


Abstract
Escherichia coli Nissle 1917 (EcN) has transformed from a traditional probiotic into a versatile microbial cell factory through innovations in genomic tools and metabolic engineering. This review summarizes recent progress in utilizing EcN for biochemical synthesis. First, the development of genetic editing tools is systematically discussed, highlighting how these methods serve as the foundation for metabolic rewiring. Second, we examine EcN bioproduction capabilities, including its application as in situ Live Biotherapeutic Products (LBPs) for targeted disease interventions and its use in the ex vivo biosynthesis of pharmaceuticals and nutraceuticals. Third, optimization strategies for fermentation processes, focusing on diverse carbon source assimilation and industrial scale-up parameters, demonstrate the potential of this strain for commercial production. Through these advancements, EcN emerges as a practical platform for next-generation biomanufacturing and precision medicine.
1. Introduction
1.1. Escherichia coli Nissle 1917 (EcN)
Escherichia coli Nissle 1917 (EcN) stands as one of the most thoroughly characterized probiotic bacterial strains, whose applications span from early 20th-century clinical practice to modern synthetic biology. Belonging to the O6:K5:H1 serotype, this strain was discovered during World War I by Dr. Alfred Nissle from a German soldier uniquely resistant to severe diarrhea [1]. Demonstrating potent antagonism against enteric pathogens, EcN was commercialized under the brand Mutaflor® [2] in 1932 and has since been extensively prescribed for various gastrointestinal disorders, including irritable bowel syndrome and Crohn’s disease [3,4,5,6].
Genomic analyses have revealed that EcN possesses a fully sequenced chromosome of approximately 5.023 megabase pairs, encompassing 5192 predicted coding sequences and several large genomic islands [7,8]. These islands encode various fitness factors, including microcins, adhesins, and multiple iron uptake systems, which contribute to the probiotic properties of EcN. In addition, EcN harbors two native cryptic plasmids, pMUT1 (3.2 kb) and pMUT2 (5.5 kb), which are stably maintained in the host strain [9,10]. Notably, the absence of classical virulence determinants distinguishes EcN from pathogenic E. coli strains [11].
1.2. Advancements in Engineering EcN: From Live Therapeutics to Industrial Cell Factories
In recent years, with advances in genomic tools and metabolic engineering, EcN has transformed from a traditional probiotic into a versatile microbial cell factory. Owing to its high genetic similarity to laboratory strains such as K-12, a wide array of established gene editing tools have been successfully adapted for the precise modification of EcN [12]. Although native EcN sometimes exhibits relatively low heterologous protein expression, strategies such as integrating T7 RNA polymerase systems have enabled EcN to achieve protein expression levels comparable to industrial strains such as BL21(DE3) [13,14].
By leveraging its inherent probiotic properties, particularly its natural propensity to colonize the tumor microenvironment [15], EcN has been engineered to function as Live Biotherapeutic Products (LBPs) [16]. As an in situ “living medicine,” its role as a gastrointestinal probiotic enables the production of antimicrobial peptides and therapeutic drugs to treat host diseases [17,18,19], while its tumor-colonizing ability facilitates the localized synthesis of anticancer drugs and diagnostic biomarkers [20]. Another approach involves utilizing EcN as a microbial cell factory for ex vivo production of pharmaceuticals and nutraceuticals. An advantage of EcN over other E. coli strains is its superior safety profile, specifically that the immunotoxicity of its lipopolysaccharide (LPS) is only 0.86% of that found in strain BL21(DE3) [13]. This significantly lower endotoxin activity minimizes the risk of residual toxicity and adverse immune responses in final products, making EcN a suitable host for the production of high-purity food- and pharmaceutical-grade metabolites [21]. Furthermore, EcN exhibits growth performance comparable to model strains such as MG1655 under both normal and stressful conditions, including thermal, acidic, and osmotic stresses. This makes it a suitable host for large-scale fermentation [22].
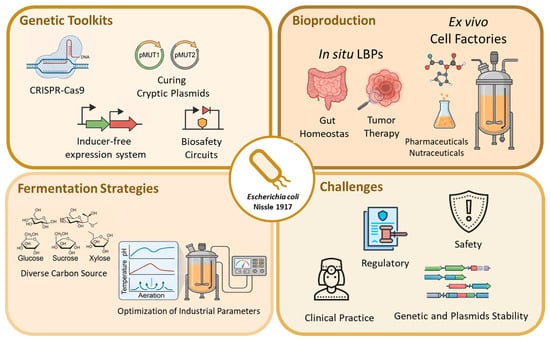
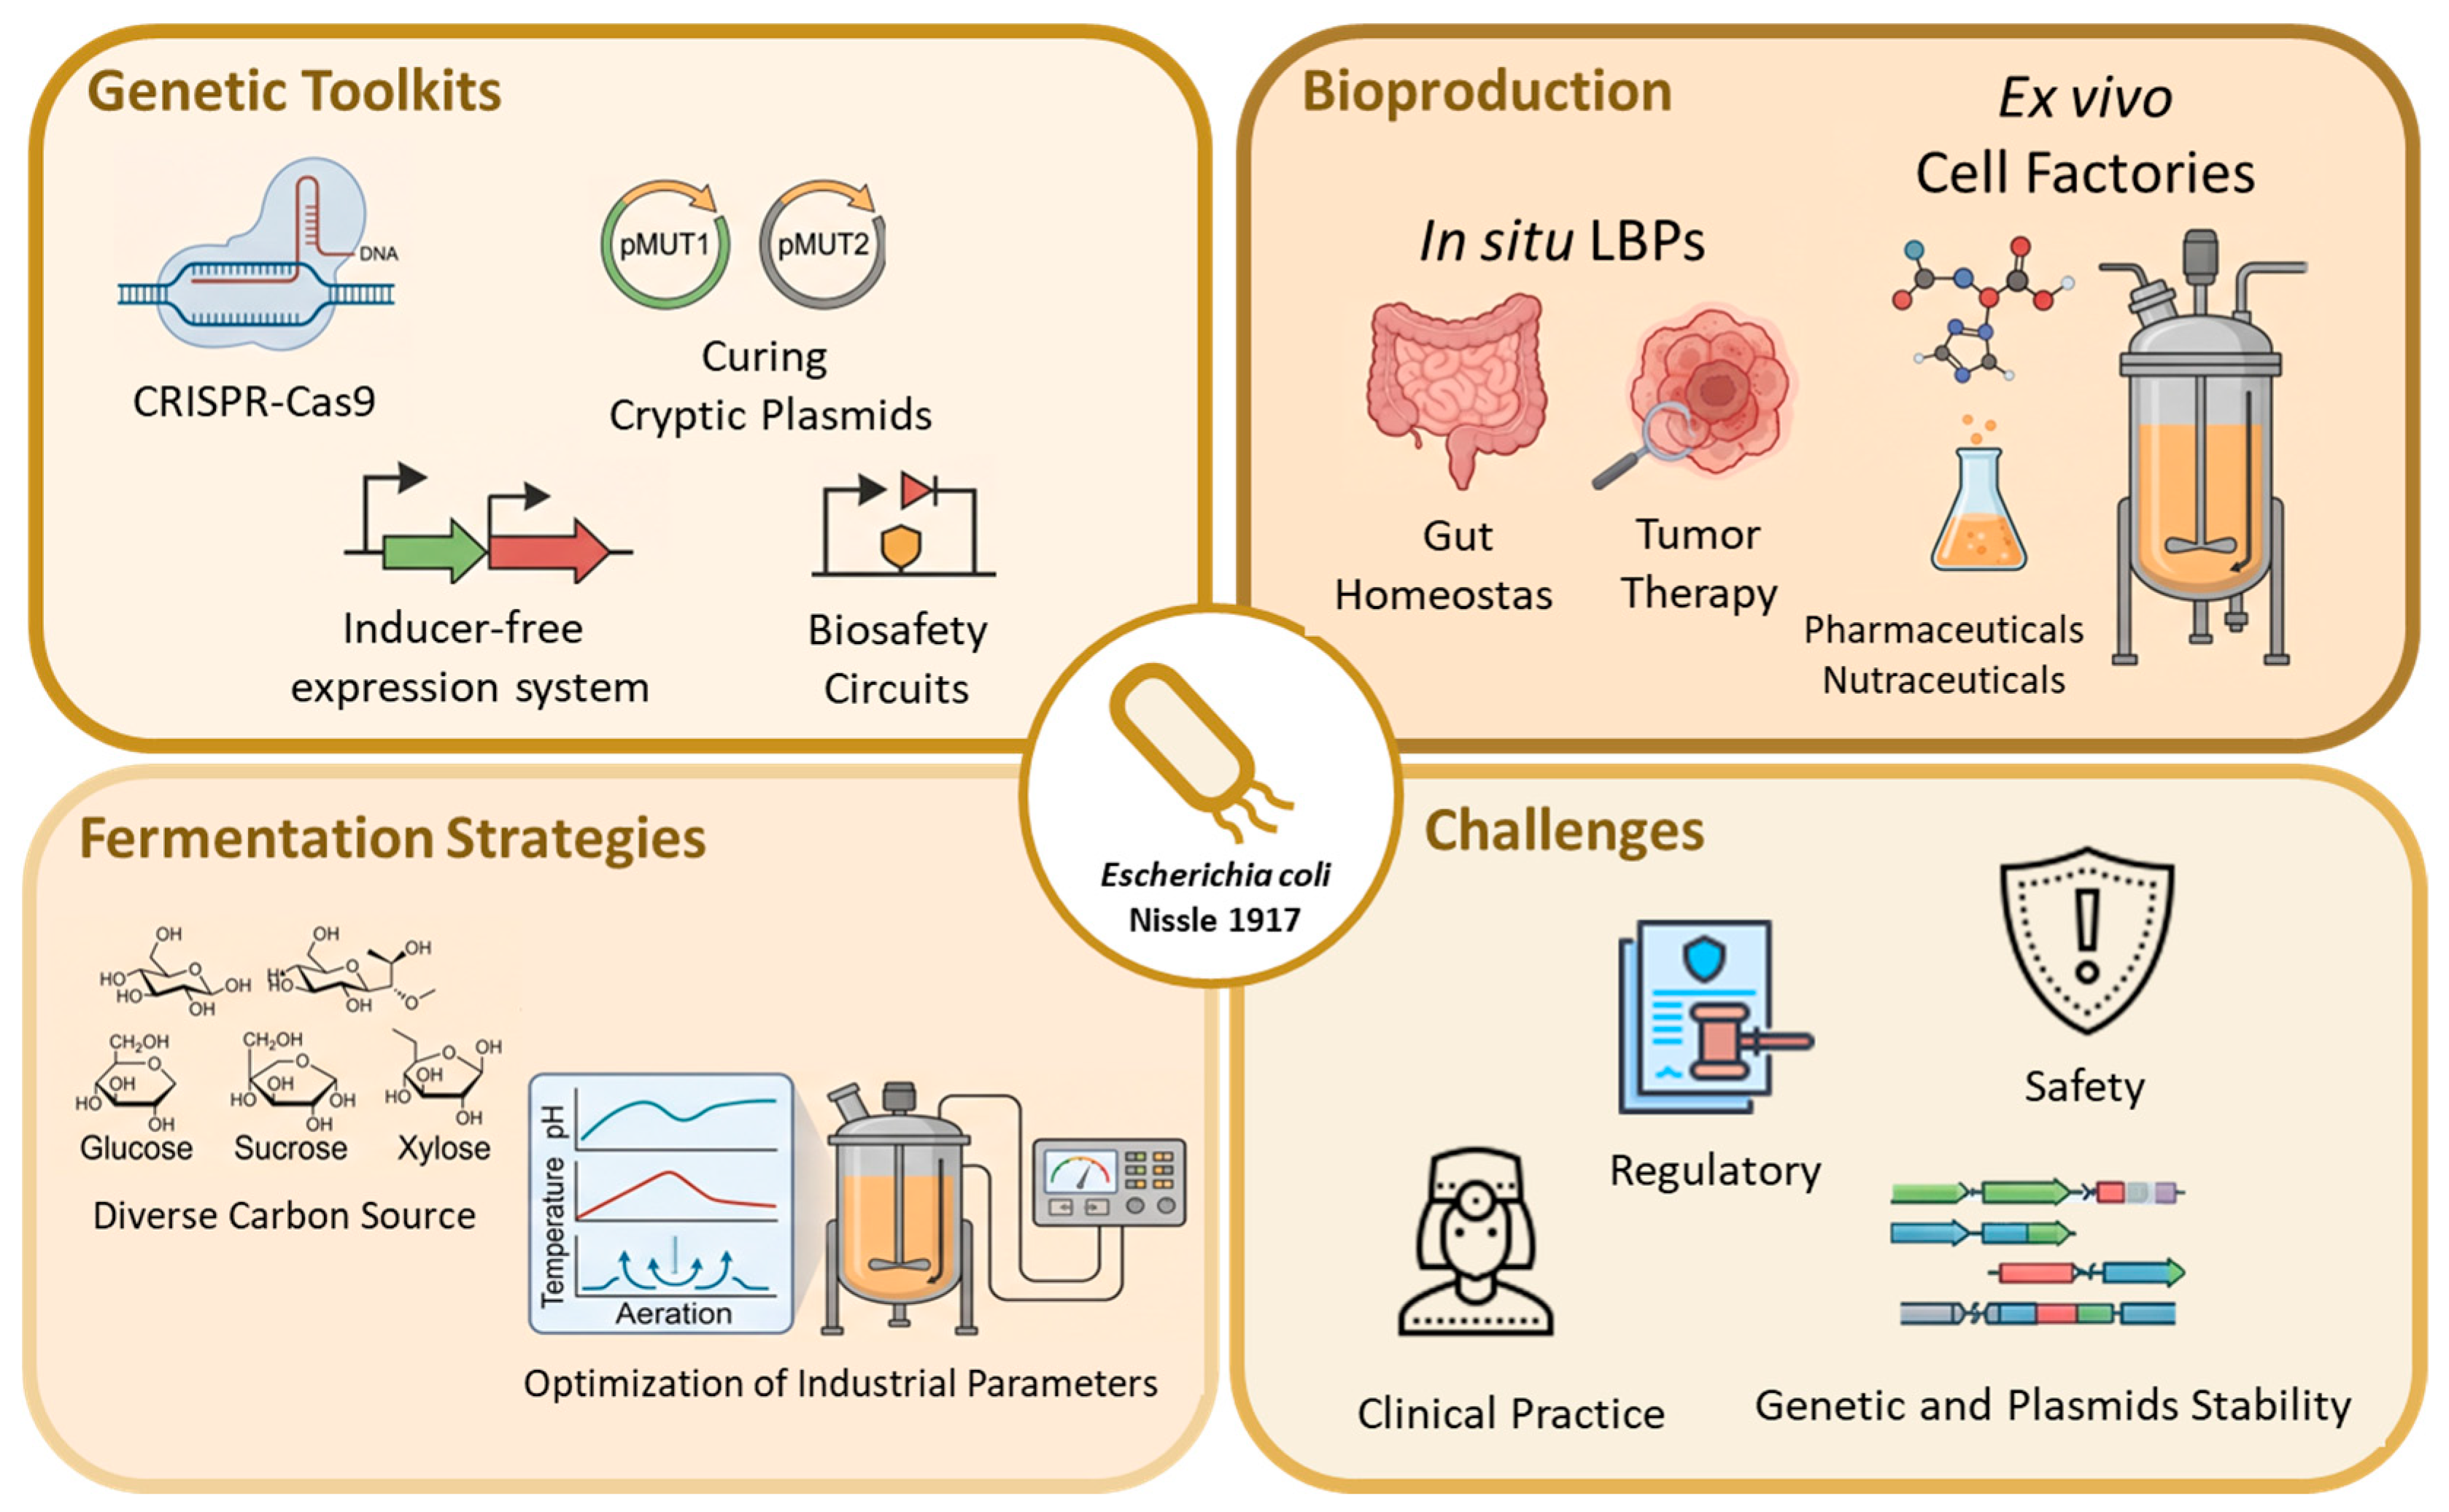
While several recent reviews have discussed the biomedical applications of engineered probiotics, a comprehensive summary that connects genetic tools, production titers, and industrial bioprocessing parameters is still lacking. This review provides an overview of the current state of EcN development through metabolic engineering for product synthesis (Figure 1). We discuss advances in genetic editing tools, reported product titers, and strategies for optimizing fermentation processes, highlighting the potential of EcN in biomanufacturing.
Figure 1.
Schematic diagram of the transition of EcN into a versatile microbial cell factory.
2. Genetic Toolkits in EcN
As a member of the Escherichia coli species, EcN shares a high degree of genetic homology with model laboratory strains, enabling the adaptation of well-established genetic editing tools for its metabolic engineering. This section discusses the versatile genetic toolkits and strategies that have been successfully employed in EcN.
2.1. Plasmid-Based Expression
Plasmid-based gene expression is a strategy that facilitates the rapid prototyping and combinatorial testing of diverse genetic designs. However, its application in EcN is complicated by the presence of endogenous plasmids. Furthermore, to comply with stringent regulatory standards for LBPs and food safety, the establishment of antibiotic-free plasmid systems is necessary. Accordingly, this section discusses current strategies for optimizing plasmid-based expression and improving vector stability. The information is summarized in Table 1.
Table 1.
Plasmid engineering approaches in engineered EcN cell factories.
2.1.1. Knockout Endogenous Plasmid pMUT1/pMUT2
EcN naturally harbors two non-essential cryptic plasmids, pMUT1 and pMUT2, which exhibit remarkable plasmid stability and minimal impact on overall cell growth [23]. Their ColE1-like replication origins cause plasmid incompatibility during metabolic engineering and hinder the introduction of standard heterologous expression vectors such as the pUC or pET series. Because traditional removal strategies such as prolonged heat stress or chemical curing are inefficient and may introduce unintended genomic mutations, targeted genetic engineering approaches are used to eliminate both plasmids.
Early studies used a selection and counter-selection method to eliminate pMUT1 and pMUT2 [30]. With advances in CRISPR-Cas9 technology, single-guide RNA (sgRNA) was initially used to target replication (rep) genes [23]. Subsequent studies optimized CRISPR strategies by shifting targets to non-essential mobilization (mob) genes. Dual-targeting sgRNAs were also used to directly cure plasmids without prior cassette insertion [24], or to simultaneously target two distinct replication sites [9].
2.1.2. Heterologous Expression Using Cryptic Plasmids
While conventional plasmids enable rapid vector prototyping, maintaining their stability in vivo without antibiotic selection remains a challenge for clinical translation. Consequently, research has shifted toward the endogenous cryptic plasmids of EcN, pMUT1 and pMUT2 [25,26,27]. These native, antibiotic-free vectors impose minimal metabolic burden [9], show high host compatibility [29], and exhibit strong plasmid stability [23]. This stability is supported by innate maintenance mechanisms, including toxin–antitoxin systems such as those present in pMUT2, which help prevent plasmid loss in the gut environment. These native vectors have been used for diverse production applications, including in vivo secretion of functional curli proteins [9] and the production of microcin L [14], phenylalanine [26], and GABA [24], without the need for antibiotic resistance markers. Furthermore, plasmid minimization has been explored as a strategy to enhance plasmid stability. pMUT1 and pMUT2 were minimized by removing genetic elements that negatively affect stability, such as the nikA and mob genes. By permanently eliminating these components, the engineered plasmids pMUT1NRΔ and pMUT2HBCΔ were constructed. These minimized plasmids maintained stability for 8 days and 12 days of continuous cultivation, respectively [29].
2.1.3. Increasing Plasmid Stability Using Auxotroph Platform
Auxotrophic platforms have been used to establish stable and safe production systems. Recently, standard auxotrophic strains, such as thymidine auxotrophs [31] (thyA knockout) and N-acetyl-D-glucosamine auxotrophs [32] (glmS knockout), have been constructed. However, relying solely on these auxotrophs is often ineffective in the complex gut microenvironment because engineered bacteria can obtain the missing nutrients from the host diet or neighboring microbes. Therefore, double knockout strategies have been used to couple these auxotrophs with essential intracellular core genes such as infA, an essential translation initiation factor, or nadE, an NH3-dependent NAD synthetase [28]. This approach provides stronger selection pressure and improves stability for clinical and industrial applications.
2.2. Chromosomal Integration and Expression
To construct robust EcN cell factories for industrial applications, achieving long-term genetic stability without continuous antibiotic selection is essential. Consequently, advanced chromosomal engineering approaches have emerged. An overview of tools and methodologies used for these chromosomal modifications is presented in Table 2.
Table 2.
Chromosomal gene expression in EcN.
2.2.1. Chromosomal Gene Integration and Gene Deletion
While episomal platforms have been optimized, chromosomal integration is increasingly used to achieve stable gene expression without selection pressure. One approach is the one-step cloning and chromosomal integration of DNA (OSIP) system, which integrates large expression cassettes into the EcN genome through phage attachment sites. Recently, this method was combined with the FLP/FRT recombination system to remove antibiotic markers and integrate the T7 RNA polymerase system into the EcN chromosome, generating a marker-free strain for recombinant production [33].
Beyond large-scale gene insertion, targeted permanent genome editing via CRISPR-Cas and λ-Red recombination systems has been utilized to knock out specific proteases (e.g., ompT) and metabolic repressors (e.g., iclR, arcA). This strategy creates streamlined chassis that improve therapeutic protein accumulation [34]. However, traditional CRISPR-based editing in EcN faces several challenges. One major limitation of the standard SpCas9 nuclease is its reliance on cytotoxic double-strand breaks (DSBs), which can result in an escaper mutation rate of up to 26% [40], unpredictable off-target effects, and cellular toxicity [39]. To overcome this limitation, Prime Editing (PE) was introduced into EcN [39]. This DSB-free and antibiotic-resistance-free workflow enables precise DNA insertions and substitutions while minimizing off-target effects during genome engineering. Furthermore, the large size of traditional SpCas9 imposes a substantial metabolic burden on the host [37], which limits the capacity for integrating complex genetic circuits. To address this size constraint, a miniaturized Type II-C CRISPR system based on Bifidobacterium-derived BLCas9 was introduced [37]. Due to its compact size, BLCas9 reduces host cellular stress and alleviates payload limitations, enabling the efficient construction of complex γ-aminobutyric acid (GABA) production pathways for gut–brain neuromodulation.
2.2.2. Modulation of Chromosomal Gene Expression
Furthermore, instead of deleting genes, CRISPR interference (CRISPRi) can be used as a reversible approach to temporarily silence gene expression. This is useful for targeting essential genes or redirecting metabolic flux. By using a catalytically inactive Cas9 (dCas9) that binds to DNA without inducing double-strand breaks, CRISPRi enables tunable and multiplexed gene repression. One application of this system is the dynamic control of gut colonization. By temporarily repressing biofilm-associated regulators (e.g., csgD) [34] and silencing specific toxin–antitoxin modules (e.g., ccdAB, hipAB) [35], the accumulation of persistent bacterial subpopulations can be effectively reduced. Ultimately, this tunable control prevents EcN from overcolonizing, thereby reducing local host tissue inflammation while ensuring safe and transient therapeutic delivery.
2.3. Promoter Systems for Transcriptional Regulation
The selection and optimization of promoter systems are essential for controlling transcription and maximizing target product yields. A summary of these transcriptional control strategies is provided in Table 3.
Table 3.
Different gene expression promoters in EcN.
To achieve high expression levels, the T7 promoter system was employed to drive protein expression upon chemical induction [33,41]. However, since EcN is being developed as both a LBPS and a platform for large-scale biomanufacturing, its engineering is shifting toward dual-free systems without antibiotics or inducers. To address this, constitutive promoters with varying strengths have been used to fine-tune transcription. Recent studies have reported screening of the J-series constitutive promoter library in EcN. Using the strong J23100 promoter to control the gadB gene enabled continuous, inducer-free γ-aminobutyric acid (GABA) production [24].
Furthermore, to decouple biomass accumulation from the production phase without chemical inducers, dynamic metabolic auto-induction systems have been developed that leverage endogenous catabolite repression. For example, an autonomous induction cascade is triggered when glucose is fully depleted [13]. For stable and chemical-free temporal control, CRISPR-assisted integration has been used to embed thermo-switchable circuits into the EcN chromosome. In this system, heterologous expression remains off during growth at 37 °C and is induced by shifting the temperature to 42 °C in the bioreactor [42].
3. Metabolic Engineering for Bioproduction
Leveraging the genetic toolkits described above, EcN has been engineered to produce a range of value-added compounds. Its ability to function as both a gut-colonizing probiotic and a low-endotoxin microbial chassis has expanded its applications in biomedical and industrial fields. This section reviews recent progress in engineered EcN, divided into two categories: LBPs for in situ treatment and ex vivo production of pharmaceuticals and nutraceuticals.
3.1. Engineered Live Biotherapeutic Products (LBPs) for In Situ Treatment
Leveraging its safety profile, native immunomodulatory properties, and ability to colonize the human gastrointestinal tract, EcN has emerged as a platform for LBPs [43]. Instead of relying on external manufacturing, engineered LBPs can detect local disease signals and deliver therapeutic molecules in situ. As summarized in Table 4, applications of engineered EcN are categorized by the therapeutic agents they produce or express. The compiled data represent current experimental findings, which are primarily at the in vitro and animal model stages.
Table 4.
Engineered Live Biotherapeutic Products (LBPs) for In Situ Treatment.
3.1.1. Tumor-Targeting and Anticancer Therapeutics
EcN can preferentially colonize hypoxic and necrotic regions within solid tumors, where immune clearance is limited [15]. This property has been used to develop EcN-based LBPs for cancer therapy. In preclinical studies, engineered EcN strains have been designed to produce and release anticancer agents within the tumor microenvironment, offering a strategy to reduce systemic toxicity associated with conventional chemotherapy.
For instance, EcN has been engineered to secrete the pro-apoptotic protein azurin [44,45], which inhibits the proliferation of colon cancer cells. Similarly, delivery of the pore-forming toxin HlyE [46] and the angiogenesis inhibitor Tum-5 [47] has shown efficacy in reducing tumor volumes in colorectal cancer and melanoma xenograft models, respectively. In addition, EcN can synthesize chemotherapeutic agents in situ, such as the histone deacetylase inhibitor romidepsin (FK228) [48], which helps mitigate its inherent cardiotoxicity, as well as secondary metabolites including colibactin, glidobactin, and luminmide, which suppress head and neck squamous cell carcinomas [49]. In combinatorial approaches, engineered EcN producing 5-aminolevulinic acid (5-ALA) [50] or L-arginine [31,51] has been combined with photodynamic and photothermal immunotherapies to eradicate solid tumors. Furthermore, in situ production of the short-chain fatty acid butyrate [52] by metabolically engineered EcN has shown anti-inflammatory and antitumor effects, reducing colorectal tumor volumes by up to 70% in murine models.
3.1.2. Bioscavengers and Delivery Vehicles for Systemic Disorders
Beyond localized solid tumors, engineered EcN serves as an in vivo bioreactor for managing systemic metabolic and neurological disorders. By continuously secreting therapeutic peptides, delivering metabolic precursors, or scavenging toxic metabolites within the gastrointestinal tract, these LBPs offer a non-invasive alternative to conventional systemic drug administration.
A prominent clinical milestone is the development of engineered EcN by Synlogic® for the treatment of phenylketonuria (PKU) [26,53]. Acting as bioscavengers, these strains are engineered to express phenylalanine ammonia-lyase (PAL) and L-amino acid deaminase (LAAD), degrading neurotoxic phenylalanine in the gut and establishing a paradigm for LBP industrialization. Furthermore, EcN has been engineered as a delivery vehicle for other metabolic conditions, including secretion of glucagon-like peptide-1 (GLP-1) [54], an incretin hormone that stimulates insulin secretion. This in situ production has been shown to alleviate hyperglycemic symptoms in both type 1 and type 2 diabetes murine models. In addition, engineered EcN has been used as an autonomous delivery system for L-DOPA in neurological disorders [55]. By synthesizing this dopamine precursor directly in the gut, the engineered strain reduced both motor and nonmotor behavioral deficits in Parkinson’s disease models, highlighting the potential of LBPs to modulate the gut–brain axis.
3.1.3. Intestinal Homeostasis and Pathogen Inhibition
EcN naturally outcompetes enteric pathogens and supports mucosal health, and synthetic biology has further enhanced these properties for targeted intestinal therapies. To address inflammatory mucosal damage, EcN has been engineered to express trefoil factors (TFFs) [56], which improve intestinal barrier function and promote epithelial repair. In addition, EcN has been engineered to overproduce antimicrobial peptides such as microcin C [57] to combat bacterial infections. The uptake of microcin C depends on specific peptide transporters, such as the YejABEF permease, which are mainly expressed by closely related enteric pathogens. This selectivity enhances bactericidal activity against target pathogens while sparing much of the commensal microbiome.
3.2. Ex Vivo Biomanufacturing of Pharmaceuticals and Nutraceuticals
Beyond its application as an in situ therapeutic, EcN has emerged as a microbial cell factory for the ex vivo production of pharmaceuticals and nutraceuticals. Compared with traditional industrial strains, EcN offers improved safety and a favorable endotoxin profile, making it a suitable host for producing human-grade compounds. Through metabolic reprogramming, EcN enables the production of diverse bioactive molecules from renewable carbon sources, providing an alternative to conventional chemical synthesis. Table 5 summarizes these engineered strains, including their target products, genetic modifications, fermentation strategies, and reported titers, highlighting the versatility of EcN as a microbial cell factory for biomanufacturing.
Table 5.
Biosynthesis of Pharmaceuticals and Nutraceuticals. DCW (dry cell weight): the biomass concentration measured as the dry mass of cells per unit culture volume (g/L).
3.2.1. Amino Acids, Polyamines, and Their Derivatives
The first major category of EcN-derived bioproducts includes amino acids, polyamines, and related derivatives. For example, γ-aminobutyric acid (GABA) [24], an inhibitory neurotransmitter, was produced at up to 17.9 g/L by expressing the gadB gene under a strong constitutive promoter (J23100). Similarly, engineered EcN has been used for Parkinson’s disease by expressing the hpaBC operon to synthesize L-DOPA (12.25 mg/L) [55], a dopamine precursor that helps restore depleted neurotransmitter levels.
Further expansion of this pathway category includes efficient biosynthesis of β-alanine (11.9 g/L) [58], achieved using a multiplex knockout strategy (ΔcycA, ΔfumB1, ΔaspC, ΔpyK) to reduce precursor degradation and redirect carbon flux. In a separate effort, EcN has been engineered to produce 5-aminolevulinic acid (5-ALA) up to 10.74 g/L for photodynamic therapy [41], through overexpression of glutamyl-tRNA reductase (hemA) to increase flux from central glutamate metabolism. Additionally, EcN has been engineered to secrete the polyamine spermidine by overexpressing the speD and speE biosynthetic pathway together with efflux pumps [59].
3.2.2. Organic Acids and Short-Chain Fatty Acids
EcN exhibits a capacity to produce organic acids and short-chain fatty acids. Because E. coli naturally generates mixed-acid fermentation by-products such as acetate, lactate, and ethanol, high product specificity requires the removal of competing pathways. For example, in butyrate production (1.76 g/L) [52], genes involved in byproduct formation (ΔadhE, Δpta, ΔpoxB) were deleted to redirect acetyl-CoA into a synthetic reversed β-oxidation pathway. This same strategy of metabolic flux redirection enabled production of 3-hydroxybutyrate (3-HB) at 105 g/L in a fed-batch system using glucose and acetate as carbon sources [13], making it one of the highest reported product yield among EcN-derived compounds. The versatility of these engineered pathways is further shown by de novo synthesis of 3-hydroxy-3-methylbutyrate (3-HMB) [60] and high-level production of p-coumaric acid (10.3 g/L) [61], which required relieving feedback inhibition in the native tyrosine pathway (ΔtyrR, ΔpheLA).
3.2.3. Complex Carbohydrates and Biopolymers
Synthesizing structurally complex carbohydrates and high-molecular-weight biopolymers presents a metabolic challenge. Heparosan, a precursor for anticoagulant pharmaceuticals, represents as one of the most extensively studied products in EcN-based production systems. For its biosynthesis [62,72] the pentose phosphate pathway and upper glycolysis were disrupted by deleting glucose-6-phosphate dehydrogenase (Δzwf) and phosphofructokinases (ΔpfkAB), thereby redirecting carbon flux toward UDP-sugar formation. Subsequent optimization further increased the titer to 9.1 g/L. A similar strategy has been applied to human milk oligosaccharide production, such as Lacto-N-triose II (2.04 g/L) [64]. Deletion of endogenous sugar-consuming pathways (ΔendA, ΔwecB) improved precursor availability for oligosaccharide assembly, highlighting EcN’s potential in infant nutrition and gastrointestinal applications.
3.2.4. Natural Products, Lipids, and Pigments
EcN can express large and complex heterologous gene clusters, enabling the biosynthesis of plant and marine natural products. Constructing these pathways often requires strong transcription systems such as genome-integrated T7 RNA polymerase. Using this approach, EcN has been engineered to produce the plant flavonoid naringenin [65] through a multi-step pathway involving tyrosine ammonia-lyase (tal), 4-coumarate CoA ligase (4cl), chalcone synthase (chs), and chalcone isomerase (chi). In a separate strategy, the antioxidant isoflavone derivative (S)-equol [66] was produced using hypoxia-responsive promoters to activate expression under anaerobic gut-like conditions.
For the production of bioactive lipids, introduction of an EPA/DHA gene cluster from a marine bacterium enabled EcN to synthesize marine omega-3 fatty acids, achieving an eicosapentaenoic acid (EPA) titer of 31.36 mg/g CDW with trace amounts of docosahexaenoic acid (DHA) [67]. Furthermore, EcN has shown strong capability for producing pigments and signaling molecules. Optimization of the heterologous mevalonate (MVA) pathway enabled production of the antioxidant lycopene (15.24 mg/L) [68]. Separately, the redirection of heme metabolism allowed for the recombinant production of biliverdin IXβ/δ isomers [69] and linear tetrapyrroles [70]. Because these molecules function as chromophores for near-infrared (NIR) fluorescent proteins, their in situ synthesis expands the use of engineered EcN for deep tissue imaging and optogenetic control in the mammalian gut.
3.2.5. Therapeutic Peptides and Non-Ribosomal Peptides (NRPs)
This category includes the ex vivo production of therapeutic peptides and complex non-ribosomal peptides (NRPs). EcN is advantageous in this context due to its clinical safety and low endotoxin profile. For protein and peptide therapeutics, reducing degradation by endogenous proteases is important for improving product accumulation. For example, sustained production and accumulation of microcin L [14], a native antimicrobial peptide, was improved by knocking out outer membrane proteases (ΔompT) to reduce extracellular product degradation.
Furthermore, beyond their primary applications as in situ live biotherapeutics, EcN’s expression systems and ability to supply diverse amino acid precursors also enable ex vivo production of structurally complex molecules. As discussed in Section 3.1, this includes secretion of therapeutic hormones such as GLP-1 [71] using the pelB signal sequence for translocation, as well as complex non-ribosomal peptides such as the anticancer agent romidepsin (FK228) [48]. The successful production of these molecules supports EcN as a microbial cell factory that links metabolic engineering with pharmaceutical production.
4. Fermentation Strategies and Bioprocessing
While advanced metabolic engineering has enabled diverse biosynthetic pathways in EcN, translating these systems into industrially viable cell factories requires robust fermentation strategies. Unlike laboratory-scale cultivation, large-scale biomanufacturing requires optimized bioprocesses to maximize product titer, yield, and productivity while reducing metabolic burden. EcN also shows growth performance comparable to model strains such as MG1655 under both normal and stress conditions, including thermal, acidic, and osmotic stress, making it a suitable host for large-scale fermentation [22]. Building on this intrinsic resilience, this section explores the fermentation characteristics of engineered EcN, focusing on its metabolic flexibility in utilizing diverse carbon sources, optimization of bioreactor parameters, and high-cell-density fermentation (HCDF) for scalable bioproduction.
4.1. Carbon Source Utilization
Carbon source selection strongly influences microbial energy generation, redox balance, and metabolic flux distribution. The assimilation of different carbon sources determines ATP production, NADH and NADPH availability, and precursor supply. Efficient redirection of carbon flux toward target pathways is therefore essential for improving product synthesis. Although glucose is commonly used in laboratory-scale E. coli fermentation, its cost and tendency to cause carbon catabolite repression [73] limit industrial application. As a result, alternative carbon sources, including industrial feedstocks and in vivo nutrients, require engineered strains with greater metabolic flexibility. This section and Table 6 summarize the carbon sources used in engineered EcN and their corresponding products.
Table 6.
Overview of carbon source utilization and metabolic engineering strategies.
4.1.1. Sugars (Fructose, Sucrose and Xylose)
Carbohydrates are widely used feedstocks in microbial fermentation. Studies show that wild-type EcN exhibits different growth profiles depending on the substrate. Glucose, fructose, and xylose support moderate growth, while glycerol results in higher biomass due to efficient uptake and metabolism via glycerol kinase and glycerol-3-phosphate dehydrogenase [41]. In contrast, EcN cannot naturally use sucrose as a sole carbon source. Although these utilization patterns are generally similar to those of standard laboratory E. coli strains, some metabolic differences remain. This section summarizes the metabolic engineering strategies used to enable the use of different sugars for bioproduction.
Fructose is an efficient alternative carbon source for microbial fermentation. It has been used to support the production of 5-aminolevulinic acid (5-ALA) in engineered EcN [41]. During production, fructose supported both cell growth and biosynthesis more effectively than glucose. EcN also shows strong fructose assimilation capacity, and genomic analysis suggests mutations in the fruA gene, which encodes a component of the fructose-specific phosphotransferase system (PTS). This adaptation may contribute to faster fructose metabolism compared with industrial strains such as BL21(DE3), with reduced acetate accumulation. By optimizing the 5-ALA pathway with stepwise feeding of fructose and glycine, a titer of 10.74 g/L was achieved, which is the highest reported 5-ALA production in EcN.
Sucrose is an abundant and cost-effective industrial feedstock. However, wild-type EcN cannot naturally use sucrose as a sole carbon source for growth. Although some strains such as E. coli W can metabolize sucrose via the csc operon [82], many standard strains, including EcN and E. coli K-12, lack this pathway. To overcome this limitation, EcN has been engineered to utilize sucrose by introducing heterologous sucrose-6-phosphate hydrolase (sacA) and sucrose phosphorylase (spl) [74]. This engineered sucrose metabolism has been applied to support heparosan production. By combining this capability with carbon flux rewiring, a heparosan titer of 622 mg/L was achieved.
Xylose, an abundant pentose in lignocellulosic biomass, represents an underexplored carbon source for EcN biomanufacturing. Although native EcN can assimilate xylose, its use as a primary carbon source in engineered EcN production systems has not yet been reported. Harnessing xylose offers the potential to utilize low-cost agricultural residues and develop orthogonal, inducer-free regulatory systems, representing a promising direction for future research.
4.1.2. Glycerol
Among non-canonical carbon sources, glycerol is a highly reduced C3 substrate and serves as an efficient carbon and energy source for EcN. Its assimilation generates more reducing equivalents (NADH) than glucose, supporting biomass accumulation. EcN has been used to produce secondary metabolites such as iron-scavenging catecholate siderophores and yersiniabactin [75]. Higher production titers have been observed when glycerol is used instead of glucose. This improvement is associated with reduced carbon catabolite repression compared with glucose. Functionally, increased production of iron chelators can limit iron availability to enteric pathogens, supporting EcN activity in the gut microbiome.
4.1.3. Short-Chain (C1/C2) Feedstocks and Mixed Carbon Co-Utilization
In the context of a circular bioeconomy, engineering EcN to utilize short-chain non-canonical carbon sources is an important objective. Acetate (C2), derived from syngas fermentation or industrial waste, is a low-cost and sustainable substrate. However, assimilation of acetate through the glyoxylate shunt and gluconeogenesis is slow and requires substantial ATP input. To address these limitations, mixed-carbon co-feeding strategies have been used. By keeping glucose at growth-limiting levels, engineered EcN can reduce carbon catabolite repression and co-assimilate both substrates. In this system, glucose catabolism provides ATP and reducing power to support acetate utilization, improving growth and enabling a 105 g/L titer of 3-hydroxybutyrate (3-HB) [13].
Pushing the boundaries of synthetic metabolism further, engineering efforts have targeted sustainable feedstocks such as CO2 and other C1 compounds. To enable CO2 utilization, the Calvin–Benson–Bassham (CBB) cycle was introduced into EcN as a CO2 recycling module. Co-expression of RuBisCO (ribulose-1,5-bisphosphate carboxylase/oxygenase) and PRK (phosphoribulokinase), together with glycerol fermentation, allowed the engineered strain to recapture fermentation-derived CO2 and increase GABA yield by 14% [76]. Similarly, efforts have been made to construct a synthetic methylotrophic EcN capable of using methanol and formate [77]. This was achieved by introducing a heterologous ribulose monophosphate (RuMP) pathway for C1 assimilation. However, despite adaptive laboratory evolution, growth remains limited when methanol or formate is used as the sole carbon source [77]. Overall, these early-stage C1 assimilation strategies still require further optimization, but they provide a foundation for expanding EcN substrate utilization toward sustainable biomanufacturing.
4.1.4. Host-Derived and Dietary Carbon (In Vivo Sources)
When deployed as an LBPs, EcN’s survival and activity depend on its ability to utilize alternative nutrients in the gastrointestinal tract. One example is ethanolamine (EA), derived from intestinal epithelial membrane turnover. EcN metabolizes EA via the eut bacterial microcompartment pathway, producing ammonium as a byproduct. However, ethanolamine ammonia-lyase requires vitamin B12, and EcN cannot use EA under B12-deficient conditions [78]. Based on this, recent studies have used the native EA-inducible eut promoter to construct a biosensor coupled with a fluorescent reporter (mRuby2), which is activated only in the presence of both EA and B12, demonstrating condition-specific gene sensing that may be useful for future LBPs. In addition, EcN metabolizes intestinal 6-deoxyhexose sugars such as L-rhamnose and L-fucose, converting lactaldehyde to 1,2-propanediol under both aerobic and anaerobic conditions [79]. This fermentative metabolism supports robust gut colonization.
Beyond host-derived compounds, EcN has been engineered or evolved to metabolize specific dietary components to establish a defined metabolic niche and outcompete endogenous gut microbes. For example, adaptive laboratory evolution has enabled EcN to use the rare sugar substitute D-allulose as a sole carbon source [80]. In addition, EcN can assimilate plant-derived sulfolipids such as sulfoquinovose (SQ) via the sulfo-EMP pathway, which is associated with yih gene variants [81]. Understanding and optimizing these scavenging pathways is important for developing LBPs that can stably colonize and function in the human gut microbiome.
4.2. Optimization of Fermentation Parameters and Scale-Up
Following metabolic rewiring of the cellular chassis, transitioning from laboratory-scale proof of concept to industrial biomanufacturing requires optimization of fermentation conditions. Because EcN shares strong physiological similarity with conventional E. coli industrial strains, most bioprocessing strategies are adapted from established E. coli protocols. As a result, the literature focused specifically on EcN bioreactor optimization remains limited. At present, EcN-derived biomanufacturing is mainly at the research and development stage, with most studies conducted in laboratory-scale bioreactors of only a few liters. One notable exception is the recent scale-up of heparosan biosynthesis [83], which demonstrated pilot-scale fermentation reaching high optical densities. Based on small-scale studies and this scale-up example, the following subsections discuss how control of physical parameters, feeding strategies, and media composition is important for advancing EcN toward industrial application.
4.2.1. Physical Parameters: Temperature, pH, and Dissolved Oxygen
Consistent with standard E. coli cultivation protocols, control of physical parameters such as temperature, pH, and dissolved oxygen (DO) is essential for stabilizing EcN growth and optimizing product titers. As summarized in Table 7, recent laboratory-scale fermentations show consistent operational ranges across different target products. Cultivation temperature is typically maintained at 37 °C. To counteract acidification caused by organic acid accumulation during active carbon metabolism, pH is controlled within a narrow range of 6.7 to 7.0. Ammonium hydroxide is commonly used for automated pH control and provides an additional nitrogen source to support sustained growth during fed-batch cultivation.
Table 7.
Summary of quantitative physical parameters in engineered EcN fermentations.
Regarding oxygen mass transfer, different operational strategies have been used to meet the respiratory demands of engineered strains. Most fed-batch processes use feedback control loops to maintain dissolved oxygen (DO) at either 20% or 30% by adjusting agitation and aeration. In addition to steady state control, DO fluctuations are also used as indicators to guide feeding strategies. In some processes, the fed-batch phase is initiated when a sharp increase in DO is observed, indicating depletion of glucose in the initial batch medium [63]. Using this DO signal enables precise coordination between carbon exhaustion and nutrient feeding, helping maintain metabolic activity and avoid extended nutrient limitation.
4.2.2. Feeding Strategies and Media Formulation
Following the establishment of physical parameters, optimization of the cultivation medium is essential for maximizing biomass and product titer. As outlined in Table 8, fermentation protocols often include complex supplements such as yeast extract and tryptone to supply biosynthetic precursors and essential vitamins, which enhance cell growth. In addition, trace metal supplementation is commonly used across scale up studies. Metal ions such as Fe2+, Zn2+, and Co2+ are important for maintaining the structure and activity of overexpressed heterologous enzymes. In some processes, complex organic components are omitted to simplify downstream purification, and chemically defined media supplemented with trace metals are used instead, as shown in lacto-N-triose II production [64].
Table 8.
Summary of cultivation media and feeding strategies in engineered EcN fermentations.
Beyond the medium composition, continuous carbon supply is controlled by different feeding strategies designed to sustain long production phases. Some processes use constant-rate fed-batch feeding, such as continuously supplying 600 g/L glucose at 20 mL/h for 5-aminolevulinic acid and chondroitin biosynthesis [63,84]. Others use exponential feeding to maintain a constant specific growth rate, for example, at 0.1 h−1 for heparosan production until dissolved oxygen depletion [62].
Additionally, some feeding strategies are used to mitigate the acetate overflow effect. When excessive carbon influx exceeds the oxidative capacity of the tricarboxylic acid (TCA) cycle, carbon flux is redirected toward acetate accumulation, which inhibits growth and reduces yield. To address this, carbon-limited feeding strategies are used. For example, pulse feeding maintains low residual carbon levels, with carbon sources replenished either after complete depletion in p-coumaric acid production [61] or when a defined low threshold (4 g/L) is reached during lacto-N-triose II biosynthesis [64]. When real-time monitoring is available, feeding strategies can be further adjusted dynamically. Overall, these carbon limitation approaches help maintain metabolic activity while avoiding overflow metabolism.
4.2.3. Scale-Up Case Study: Heparosan Production
Engineered EcN biomanufacturing remains at the research stage, with no reported commercial-scale production to date. The most extensively documented scale-up is the pilot-scale production of heparosan [83]. In this study, the fermentation process was successfully transferred to a 100 L bioreactor. Using a defined medium and tight control of pH (6.8 via NH4OH) and dissolved oxygen (30% via cascaded agitation), the process minimized oxygen limitation and acetate accumulation. The engineered strain achieved an OD600 of 160–180 and a final heparosan titer of 3.0 g/L. While this study demonstrates that EcN can be operated at pilot scale, bridging the gap between 100 L processes and commercial scale manufacturing remains a challenge. Further validation of scale-up parameters and optimization of fermentation conditions will be required to support industrial deployment of EcN-based cell factories.
5. Future Perspectives and Challenges
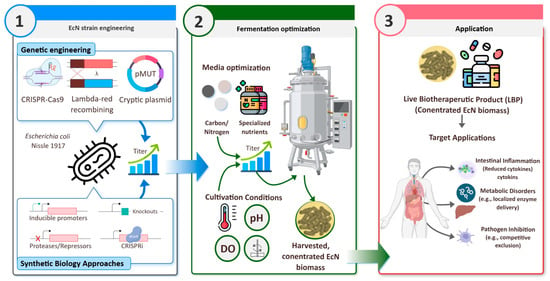
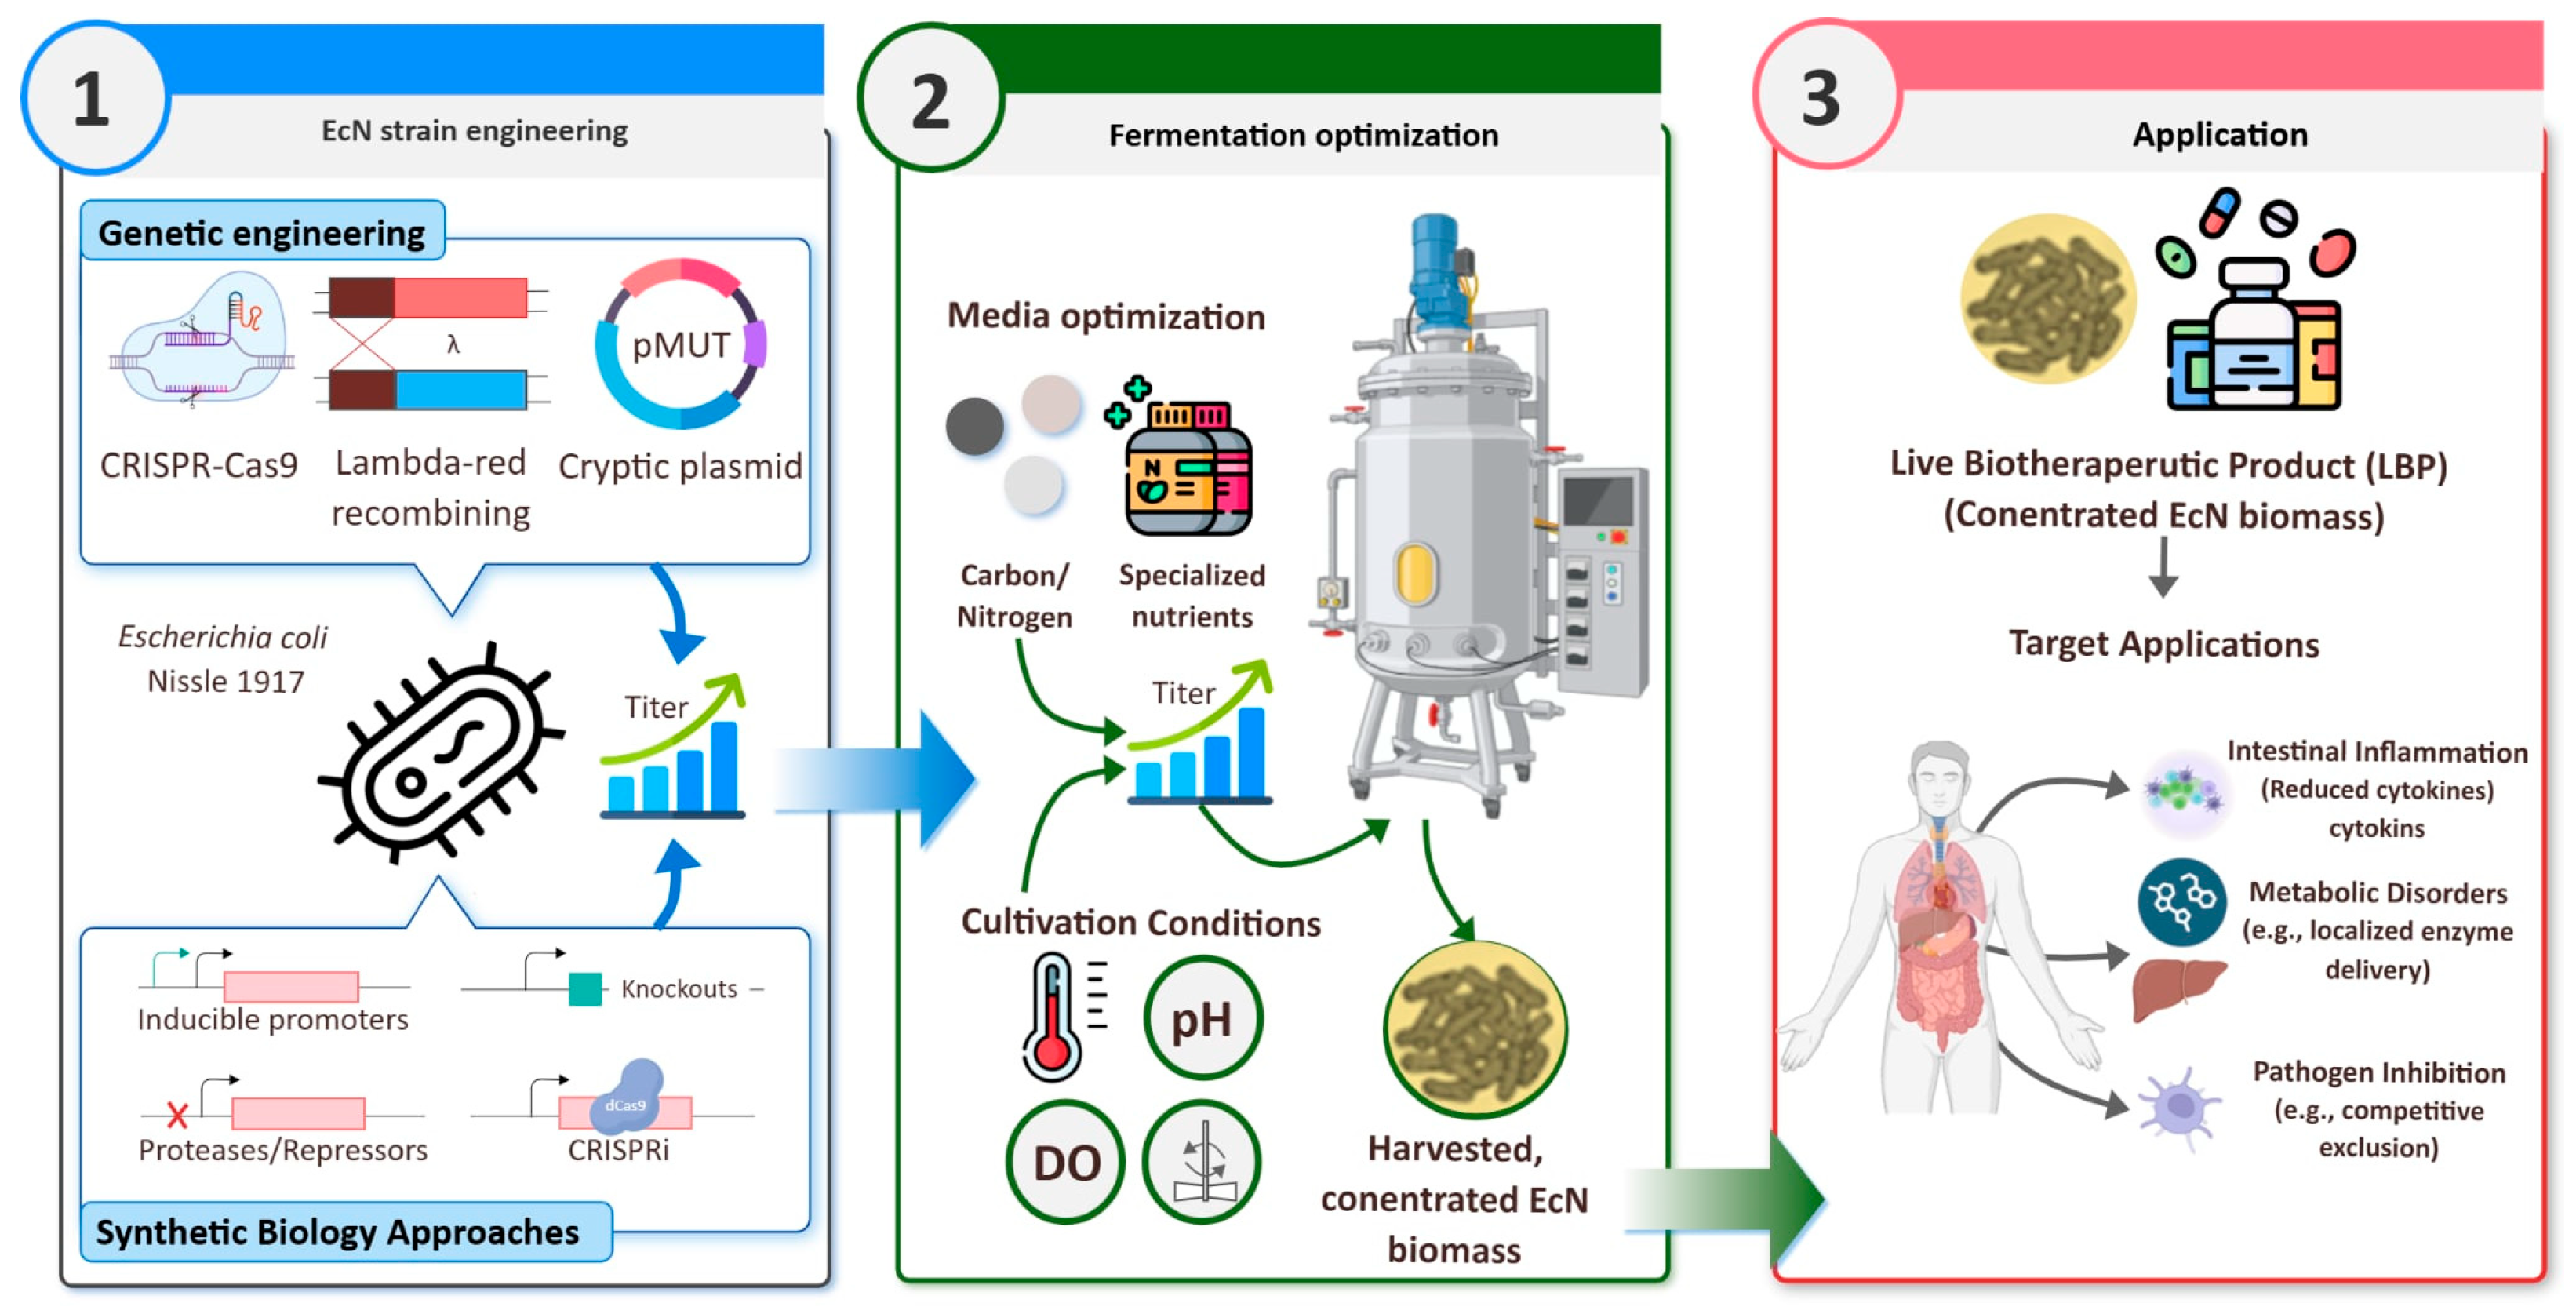
To successfully translate engineered platforms into practical settings, a coordinated development workflow linking synthetic biology approaches, cultivation parameter tuning, and final biomass harvesting is established (Figure 2).
Figure 2.
Development workflow of engineered EcN for live biotherapeutics.
Despite the progress in engineering EcN for therapeutic and industrial applications, several challenges remain in achieving full clinical and commercial use. As the field moves from proof-of-concept studies toward human application and large-scale bioprocessing, multiple limitations become more evident. This section highlights key bottlenecks in EcN research, including safety and regulatory requirements, long-term strain stability, and challenges in industrial scale-up and clinical translation.
5.1. Safety, Biocontainment, and Long-Term Genetic Stability
Translating engineered EcN into clinical applications and large-scale biomanufacturing requires addressing biosafety, regulatory, and physiological challenges. Regulatory approval for live biotherapeutic products (LBPs) is stringent and requires environmental risk assessments and compliance with FDA or EMA guidelines. A key biosafety concern is horizontal gene transfer [17,85,86], where engineered genetic circuits, particularly those involving antibiotic resistance, may spread to the native gut microbiota. In addition, shedding viable EcN in feces raises ecological concerns. A major physiological limitation is the long-term stability of engineered strains. The metabolic burden from continuous heterologous expression can impose strong selective pressure, leading to plasmid instability, mutations, or loss of synthetic pathway activity in the gut environment.
To address these challenges, researchers are combining genetic and metabolic engineering strategies. To meet biosafety requirements and reduce horizontal gene transfer risks, antibiotic resistance markers and chemical inducers should be removed. For environmental containment, fail-safe systems such as temperature-sensitive suicide switches and engineered DNA phosphorothioate-based phage defense modules have been developed to restrict cell survival to conditions similar to the human gut [42,87]. In addition, chromosomal integration of synthetic cassettes is preferred over episomal vectors to improve genetic stability and maintain expression without selection pressure. To reduce metabolic burden, dynamic regulatory systems are used to separate growth and production phases. Examples include acyl homoserine lactone-based quorum-sensing circuits [61] and stress-responsive promoters such as PuspA or PgadA that activate under nutrient limitation [88]. Together, these strategies help improve biosafety and long-term stability of engineered EcN.
5.2. Techno-Economic Feasibility and Commercialization Challenges
From an industrial and commercialization perspective, the techno-economic feasibility of EcN cell factories remains a key challenge. Although current pilot-scale studies demonstrate technical feasibility, large-scale commercialization is limited by economic constraints. Product titers and substrate-to-product yields achieved at laboratory and pilot scales are often insufficient for cost-effective industrial production. Improving economic performance will require continued metabolic optimization to increase fermentation productivity, as well as the use of cost-effective chemically defined media to reduce raw material and downstream processing costs.
Beyond bioprocessing economics, EcN presents additional commercial challenges. Because engineered EcN is often developed as LBPs or oral functional supplement, its commercialization is governed by strict regulatory frameworks. These include preclinical safety evaluation, phased clinical trials, and compliance with good manufacturing practice (GMP), all of which require substantial cost and long development timelines. As a result, techno-economic analysis (TEA) will be important early in development to identify major cost drivers, improve fermentation performance, and account for clinical translation costs, helping to bridge the gap between laboratory-scale engineering and economically viable commercialization.
5.3. Translation: From Laboratory Proof-of-Concept to Clinical Reality
Despite advances in metabolic engineering, most engineered EcN systems remain at the laboratory proof-of-concept stage. For industrial production, further optimization of scale-up fermentation parameters is required, extending beyond the high-density conditions demonstrated in heparosan production, to support a broader range of newly synthesized products.
While the studies described above demonstrate the biochemical capabilities of EcN in controlled laboratory settings, their relevance to human applications remains uncertain. More importantly, clinical translation of engineered EcN as LBPs requires extensive human trials, which carry a substantial risk of failure. An example of this translational gap occurred in early 2024 when Synlogic®, a pioneering company in LBP development, was forced to halt operations after its lead engineered EcN candidate for phenylketonuria (SYNB1934) failed to meet primary efficacy endpoints in a pivotal Phase 3 clinical trial. This limitation highlights that, although animal models often show strong therapeutic effects, robust clinical data are essential to validate the pharmacokinetics, colonization stability, and in vivo functionality of genetically modified EcN in the complex human gastrointestinal tract.
6. Conclusions
In conclusion, EcN has emerged as a valuable platform in synthetic biology. It combines the genetic tractability of an industrial microbe with the safety profile and immunomodulatory properties of a probiotic, making it a versatile chassis. While challenges in genetic stability, biocontainment, and regulatory approval remain, advances in CRISPR-based genome editing, dynamic metabolic control, and scale-up bioprocessing are gradually addressing these barriers. To fully realize its industrial potential, remaining bottlenecks, such as acetate overflow during high-cell-density fermentation and the economic constraints of live biotherapeutic products (LBPs), must still be overcome. Furthermore, integrating AI-guided metabolic modeling and comprehensive techno-economic analysis (TEA) will be important for bridging the gap between laboratory success and commercial viability. Ultimately, continued optimization of engineered EcN may enable advances in sustainable biomanufacturing and targeted live biotherapeutics.
Author Contributions
Conceptualization, formal analysis, investigation, data curation, writing—original draft preparation, visualization, writing—review and editing, J.J.-C.H. and T.P.-J.T.; supervision, project administration, funding acquisition, E.I.L. All authors have read and agreed to the published version of the manuscript.
Funding
This research was funded by National Science and Technology Council (NSTC), grant number NSTC 114-2321-B-A49-010 and by the Center for Intelligent Drug Systems and Smart Bio-devices (IDS2B), Smart Platform of Dynamic Systems Biology for Therapeutic Development within the framework of the Higher Education Sprout Project of the Ministry of Education.
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
No new data were created or analyzed in this study. Data sharing is not applicable to this article.
Acknowledgments
During the preparation of this manuscript, the authors used Gemini (https://gemini.google.com, accessed 15 April 2026) for the purposes of generating a few small icons within two of the schematic diagrams. The authors have reviewed, edited, and assembled these components into the final figures using Microsoft PowerPoint, and take full responsibility for the content of this publication.
Conflicts of Interest
The authors declare no conflicts of interest.
References
- Nissle, A. Die antagonistische behandlung chronischer darmstörungen mit colibakterien. Med. Klin. 1918, 2, 29–33. [Google Scholar]
- Jacobi, C.A.; Malfertheiner, P. Escherichia coli Nissle 1917 (Mutaflor): New insights into an old probiotic bacterium. Dig. Dis. 2011, 29, 600–607. [Google Scholar] [CrossRef] [Scilit]
- Schultz, M. Clinical use of E. coli Nissle 1917 in inflammatory bowel disease. Inflamm. Bowel Dis. 2008, 14, 1012–1018. [Google Scholar] [CrossRef] [Scilit]
- Sonnenborn, U.; Schulze, J. The non-pathogenic Escherichia coli strain Nissle 1917–features of a versatile probiotic. Microb. Ecol. Health Dis. 2009, 21, 122–158. [Google Scholar]
- Sonnenborn, U. Escherichia coli strain Nissle 1917-from bench to bedside and back: History of a special Escherichia coli strain with probiotic properties. FEMS Microbiol. Lett. 2016, 363, fnw212. [Google Scholar] [CrossRef] [Scilit]
- Kruis, W.; Frič, P.; Pokrotnieks, J.; Lukáš, M.; Fixa, B.; Kaščák, M.; Kamm, M.; Weismueller, J.; Beglinger, C.; Stolte, M. Maintaining remission of ulcerative colitis with the probiotic Escherichia coli Nissle 1917 is as effective as with standard mesalazine. Gut 2004, 53, 1617–1623. [Google Scholar] [CrossRef] [Scilit]
- Cress, B.F.; Linhardt, R.J.; Koffas, M.A.G. Draft genome sequence of Escherichia coli strain Nissle 1917 (serovar O6:K5:H1). Genome Announc. 2013, 1, e00047-13. [Google Scholar] [CrossRef] [Scilit]
- Reister, M.; Hoffmeier, K.; Krezdorn, N.; Rotter, B.; Liang, C.; Rund, S.; Dandekar, T.; Sonnenborn, U.; Oelschlaeger, T.A. Complete genome sequence of the gram-negative probiotic Escherichia coli strain Nissle 1917. J. Biotechnol. 2014, 187, 106–107. [Google Scholar] [CrossRef] [Scilit]
- Kan, A.; Gelfat, I.; Emani, S.; Praveschotinunt, P.; Joshi, N.S. Plasmid vectors for in vivo selection-free use with the probiotic E. coli Nissle 1917. ACS Synth. Biol. 2020, 10, 94–106. [Google Scholar] [CrossRef] [Scilit]
- Grozdanov, L.; Raasch, C.; Schulze, J.; Sonnenborn, U.; Gottschalk, G.; Hacker, J.; Dobrindt, U. Analysis of the genome structure of the nonpathogenic probiotic Escherichia coli strain Nissle 1917. J. Bacteriol. 2004, 186, 5432–5441. [Google Scholar] [CrossRef] [Scilit]
- Sun, J.; Gunzer, F.; Westendorf, A.M.; Buer, J.; Scharfe, M.; Jarek, M.; Gößling, F.; Blöcker, H.; Zeng, A.P. Genomic peculiarity of coding sequences and metabolic potential of probiotic Escherichia coli strain Nissle 1917 inferred from raw genome data. J. Biotechnol. 2005, 117, 147–161. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yu, M.; Hu, S.; Tang, B.; Yang, H.; Sun, D. Engineering Escherichia coli Nissle 1917 as a microbial chassis for therapeutic and industrial applications. Biotechnol. Adv. 2023, 67, 108202. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yang, F.-R.; Zheng, Y.; Deng, R.-Z.; Xia, L.; Wang, H.-M.; Deng, Y.-H.; Situ, W.; Xiao, Y.-C.; Shen, H.-W.; Lv, J.-Y. Hyperproduction of 3-hydroxybutyrate using engineered probiotic E. coli Nissle 1917 from glucose and CO 2-derived acetate. Green Chem. 2026, 28, 2328–2341. [Google Scholar] [CrossRef] [Scilit]
- Zainuddin, H.S.; Murali, S.K.; Mansell, T.J. Engineered stable, antibiotic-free, high-level protein expression in the probiotic chassis Escherichia coli Nissle 1917. Biotechnol. Bioeng. 2026, 123, 776–784. [Google Scholar] [CrossRef] [Scilit]
- Radford, G.A.; Vrbanac, L.; de Nys, R.T.; Worthley, D.L.; Wright, J.A.; Hasty, J.; Woods, S.L. Towards understanding tumour colonisation by probiotic bacterium E. coli Nissle 1917. Cancers 2024, 16, 2971. [Google Scholar] [CrossRef] [Scilit]
- Das, B. Live biotherapeutics in the clinic: Regulatory pathways, market dynamics, and future trends. Prog. Mol. Biol. Transl. Sci. 2026, 220, 405–416. [Google Scholar]
- Effendi, S.S.W.; Ng, I.-S. Prospective and challenges of live bacterial therapeutics from a superhero Escherichia coli Nissle 1917. Crit. Rev. Microbiol. 2023, 49, 611–627. [Google Scholar] [CrossRef] [Scilit]
- Ou, B.; Yang, Y.; Tham, W.L.; Chen, L.; Guo, J.; Zhu, G. Genetic engineering of probiotic Escherichia coli Nissle 1917 for clinical application. Appl. Microbiol. Biotechnol. 2016, 100, 8693–8699. [Google Scholar] [CrossRef] [Scilit]
- Ninyio, N.; Schmitt, K.; Sergon, G.; Nilsson, C.; Andersson, S.; Scherbak, N. Stable expression of HIV-1 MPER extended epitope on the surface of the recombinant probiotic bacteria Escherichia coli Nissle 1917 using CRISPR/Cas9. Microb. Cell Factories 2024, 23, 39. [Google Scholar] [CrossRef] [Scilit]
- Liu, Q.; Gai, Y.; Chen, Y.; Lan, X.; Jiang, D. Escherichia coli Nissle 1917 as a novel microrobot for tumor-targeted imaging and therapy. Pharmaceutics 2021, 13, 1226. [Google Scholar] [CrossRef] [Scilit]
- Wakelin, S.J.; Sabroe, I.; Gregory, C.D.; Poxton, I.R.; Forsythe, J.L.; Garden, O.J.; Howie, S.E. “Dirty little secrets”—Endotoxin contamination of recombinant proteins. Immunol. Lett. 2006, 106, 1–7. [Google Scholar] [CrossRef] [Scilit]
- Ramadevi, S.; Shelin, R.; Shanmugaraja, M. Comprehensive Analysis of the Physiological Characterization of Escherichia coli Nissle 1917. Curr. Microbiol. 2023, 80, 150. [Google Scholar] [CrossRef] [Scilit]
- Zainuddin, H.S.; Bai, Y.; Mansell, T.J. CRISPR-based curing and analysis of metabolic burden of cryptic plasmids in Escherichia coli Nissle 1917. Eng. Life Sci. 2019, 19, 478–485. [Google Scholar] [CrossRef] [Scilit]
- Lan, Y.J.; Tan, S.; Cheng, S.Y.; Ting, W.W.; Xue, C.F.; Lin, T.H.; Cai, M.Z.; Chen, P.T.; Ng, I.S. Development of Nissle 1917 derivative by CRISPR/Cas9 and application for gamma-aminobutyric acid (GABA) production in antibiotic-free system. Biochem. Eng. J. 2021, 168, 107952. [Google Scholar] [CrossRef] [Scilit]
- Forkus, B.; Ritter, S.; Vlysidis, M.; Geldart, K.; Kaznessis, Y.N. Antimicrobial Probiotics Reduce Salmonella enterica in Turkey Gastrointestinal Tracts. Sci. Rep. 2017, 7, 40695. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Isabella, V.M.; Ha, B.N.; Castillo, M.J.; Lubkowicz, D.J.; Rowe, S.E.; Millet, Y.A.; Anderson, C.L.; Li, N.; Fisher, A.B.; West, K.A. Development of a synthetic live bacterial therapeutic for the human metabolic disease phenylketonuria. Nat. Biotechnol. 2018, 36, 857–864. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Riglar, D.T.; Giessen, T.W.; Baym, M.; Kerns, S.J.; Niederhuber, M.J.; Bronson, R.T.; Kotula, J.W.; Gerber, G.K.; Way, J.C.; Silver, P.A. Engineered bacteria can function in the mammalian gut long-term as live diagnostics of inflammation. Nat. Biotechnol. 2017, 35, 653–658. [Google Scholar] [CrossRef] [Scilit]
- Amrofell, M.B.; Rengarajan, S.; Vo, S.T.; Tovar, E.S.R.; LoBello, L.; Dantas, G.; Moon, T.S. Engineering E. coli strains using antibiotic-resistance-gene-free plasmids. Cell Rep. Methods 2023, 3, 100669. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhou, S.; Zhao, L.; Zuo, W.; Zheng, Y.; Zhang, P.; Sun, Y.; Wang, Y.; Du, G.; Kang, Z. Minimizing endogenous cryptic plasmids to construct antibiotic-free expression systems for Escherichia coli Nissle 1917. Synth. Syst. Biotechnol. 2024, 9, 165–175. [Google Scholar] [CrossRef] [Scilit]
- Remer, K.A.; Bartrow, M.; Roeger, B.; Moll, H.; Sonnenborn, U.; Oelschlaeger, T.A. Split immune response after oral vaccination of mice with recombinant Escherichia coli Nissle 1917 expressing fimbrial adhesin K88. Int. J. Med. Microbiol. 2009, 299, 467–478. [Google Scholar] [CrossRef] [Scilit]
- Kurtz, C.B.; Millet, Y.A.; Puurunen, M.K.; Perreault, M.; Charbonneau, M.R.; Isabella, V.M.; Kotula, J.W.; Antipov, E.; Dagon, Y.; Denney, W.S. An engineered E. coli Nissle improves hyperammonemia and survival in mice and shows dose-dependent exposure in healthy humans. Sci. Transl. Med. 2019, 11, eaau7975. [Google Scholar] [CrossRef] [Scilit]
- Shao, F.; Wu, R.; Li, Z.J. Metabolic Engineering of Escherichia coli Nissle 1917 for the Production of Heparosan Using Mixed Carbon Sources. Fermentation 2025, 11, 289. [Google Scholar] [CrossRef] [Scilit]
- Effendi, S.S.W.; Ng, I.S. Reprogramming T7RNA Polymerase in Escherichia coli Nissle 1917 under Specific Lac Operon for Efficient p-Coumaric Acid Production. ACS Synth. Biol. 2022, 11, 3471–3481. [Google Scholar] [CrossRef] [Scilit]
- Wang, C.; Luo, L.; Dai, Z.; Zhang, W.; Ma, Y.; Wang, J. Construction of probiotic Escherichia coli Nissle 1917 as a next-generation expression platform and its application in therapeutic protein production. J. Biol. Eng. 2026, 20, 18. [Google Scholar] [CrossRef] [Scilit]
- Azam, M.W.; Khan, A.U. CRISPRi-mediated suppression of E. coli Nissle 1917 virulence factors: A strategy for creating an engineered probiotic using csgD gene suppression. Front. Nutr. 2022, 9, 938989. [Google Scholar] [CrossRef] [Scilit]
- Xu, J.; Xia, K.; Li, P.; Qian, C.; Li, Y.; Liang, X. Functional investigation of the chromosomal ccdAB and hipAB operon in Escherichia coli Nissle 1917. Appl. Microbiol. Biotechnol. 2020, 104, 6731–6747. [Google Scholar] [CrossRef] [Scilit]
- Liu, Q.; Huang, Y.; Zhou, R.; Ding, H.; Nie, Q.; Gong, X.; Zuo, T.; Wang, S.; Liang, Y.; Li, Y. A Minimal and Portable CRISPR Platform Based on Bifidobacterial Cas9 Enables Genome Editing in E. coli Nissle 1917. ACS Synth. Biol. 2026, 15, 1544–1556. [Google Scholar] [CrossRef] [Scilit]
- Fang, M.; Zhang, R.; Wang, C.; Liu, Z.; Fei, M.; Tang, B.; Yang, H.; Sun, D. Engineering probiotic Escherichia coli Nissle 1917 to block transfer of multiple antibiotic resistance genes by exploiting a type I CRISPR-Cas system. Appl. Environ. Microbiol. 2024, 90, e00811-24. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, P.-R.; Wei, Y.; Li, X.; Yu, H.-Y.; Wang, S.-G.; Yuan, X.-Z.; Xia, P.-F. Precision engineering of the probiotic Escherichia coli Nissle 1917 with prime editing. Appl. Environ. Microbiol. 2025, 91, e00031-25. [Google Scholar] [CrossRef] [Scilit]
- Widney, K.A.; Yang, D.-D.; Rusch, L.M.; Copley, S.D. CRISPR-Cas9-assisted genome editing in E. coli elevates the frequency of unintended mutations. bioRxiv 2024. [Google Scholar] [CrossRef] [Scilit]
- Hsu, C.-H.; Effendi, S.S.W.; Ting, W.-W.; Ng, I.-S. Fructose-Driven Biosynthesis of 5-Aminolevulinic Acid in the Engineered Probiotic Escherichia coli Nissle 1917. ACS Sustain. Chem. Eng. 2025, 14, 1032–1042. [Google Scholar] [CrossRef] [Scilit]
- Lin, T.-H.; Cheng, S.-Y.; Lin, Y.-F.; Chen, P.-T. Development of the low-temperature inducible system for recombinant protein production in Escherichia coli Nissle 1917. J. Agric. Food Chem. 2024, 72, 7318–7325. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sadhu, S.; Paul, T.; Yadav, N. Therapeutic engineering of the gut microbiome using synthetic biology and metabolic tools: A comprehensive review with E. coli Nissle 1917 as a model case study. Arch. Microbiol. 2025, 207, 213. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ma, Y.; Zhu, G.; Feng, L.; Jiang, S.; Xiang, Q.; Wang, J. Efficient cytotoxicity of recombinant azurin in Escherichia coli Nissle 1917-derived minicells against colon cancer cells. Bioengineering 2023, 10, 1188. [Google Scholar] [CrossRef] [Scilit]
- Zhang, Y.; Zhang, Y.; Xia, L.; Zhang, X.; Ding, X.; Yan, F.; Wu, F. Escherichia coli Nissle 1917 targets and restrains mouse B16 melanoma and 4T1 breast tumors through expression of azurin protein. Appl. Environ. Microbiol. 2012, 78, 7603–7610. [Google Scholar] [CrossRef] [Scilit]
- Chiang, C.J.; Huang, P.H. Metabolic engineering of probiotic Escherichia coli for cytolytic therapy of tumors. Sci. Rep. 2021, 11, 5853. [Google Scholar] [CrossRef] [Scilit]
- He, L.; Yang, H.; Liu, F.; Chen, Y.; Tang, S.; Ji, W.; Tang, J.; Liu, Z.; Sun, Y.; Hu, S. Escherichia coli Nissle 1917 engineered to express Tum-5 can restrain murine melanoma growth. Oncotarget 2017, 8, 85772. [Google Scholar] [CrossRef] [Scilit]
- Ma, C.; Li, G.; Sun, T.; Tang, X.; Qiu, T.; Song, J.; Wang, H.; Zhang, Y.; Jiang, T. Engineered romidepsin biosynthetic pathways in Escherichia coli Nissle 1917 improve the efficacy of bacteria-mediated cancer therapy. PLoS Biol. 2026, 24, e3003657. [Google Scholar] [CrossRef] [Scilit]
- Li, R.; Helbig, L.; Fu, J.; Bian, X.; Herrmann, J.; Baumann, M.; Stewart, A.F.; Müller, R.; Li, A.; Zips, D. Expressing cytotoxic compounds in Escherichia coli Nissle 1917 for tumor-targeting therapy. Res. Microbiol. 2019, 170, 74–79. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, J.; Li, X.; Liu, Y.; Su, T.; Lin, C.; Shao, L.; Li, L.; Li, W.; Niu, G.; Yu, J.; et al. Engineering a probiotic strain of Escherichia coli to induce the regression of colorectal cancer through production of 5-aminolevulinic acid. Microb. Biotechnol. 2021, 14, 2130–2139. [Google Scholar] [CrossRef] [Scilit]
- Hu, Q.; Huang, X.; Wang, T.; Lu, Z.; Sun, D.; Jin, Y. Engineered Probiotics-Based Biohybrid-Driven Tumor Metabolic Remodeling To Boost Tumor Photoimmunotherapy. ACS Appl. Mater. Interfaces 2025, 17, 30516–30532. [Google Scholar] [CrossRef] [Scilit]
- Chiang, C.J.; Hong, Y.H. In situ delivery of biobutyrate by probiotic Escherichia coli for cancer therapy. Sci. Rep. 2021, 11, 18172. [Google Scholar] [CrossRef] [Scilit]
- Puurunen, M.K.; Vockley, J.; Searle, S.L.; Sacharow, S.J.; Phillips, J.A., III; Denney, W.S.; Goodlett, B.D.; Wagner, D.A.; Blankstein, L.; Castillo, M.J. Safety and pharmacodynamics of an engineered E. coli Nissle for the treatment of phenylketonuria: A first-in-human phase 1/2a study. Nat. Metab. 2021, 3, 1125–1132. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Luo, J.; Fang, Y.; Qi, Z.; Cui, F.; Hu, H.; Li, S.; Chen, T.; Zhang, H. Administration of a next-generation probiotic Escherichia coli Nissle 1917-GLP-1 alleviates diabetes in mice with type 1 and type 2 diabetes. Can. J. Infect. Dis. Med. Microbiol. 2025, 2025, 6675676. [Google Scholar] [CrossRef] [Scilit]
- Abdalla, A.; Padhi, P.; Bakes, N.; Thyer, R.; Zenitsky, G.; Jin, H.; Anantharam, V.; Kanthasamy, A.; Ellington, A.D.; Phillips, G.J. Preclinical Evaluation of Synthetic Biology-Driven Engineered Escherichia coli Nissle 1917 as a Living Therapeutic for Sustained L-DOPA Delivery. ACS Synth. Biol. 2026, 15, 748–761. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Praveschotinunt, P.; Duraj-Thatte, A.M.; Gelfat, I.; Bahl, F.; Chou, D.B.; Joshi, N.S. Engineered E. coli Nissle 1917 for the delivery of matrix-tethered therapeutic domains to the gut. Nat. Commun. 2019, 10, 5580. [Google Scholar] [CrossRef] [Scilit]
- Bartram, E.; Asai, M.; Gabant, P.; Wigneshweraraj, S. Enhancing the antibacterial function of probiotic Escherichia coli Nissle: When less is more. Appl. Environ. Microbiol. 2023, 89, e00975-23. [Google Scholar] [CrossRef] [Scilit]
- Hu, S.; Fei, M.; Fu, B.; Yu, M.; Yuan, P.; Tang, B.; Yang, H.; Sun, D. Development of probiotic E. coli Nissle 1917 for β-alanine production by using protein and metabolic engineering. Appl. Microbiol. Biotechnol. 2023, 107, 2277–2288. [Google Scholar] [CrossRef] [Scilit]
- Caffaratti, C.; Plazy, C.; Cunin, V.; Toussaint, B.; Le Gouellec, A. Bioengineering of Escherichia coli Nissle 1917 for Production and Excretion of Spermidine, a Key Metabolite in Human Health. Metabolites 2022, 12, 1061. [Google Scholar] [CrossRef] [Scilit]
- Huang, S.J.; Lai, M.J.; Chen, A.Y.; Lan, E.I. De novo biosynthesis of 3-hydroxy-3-methylbutyrate as anti-catabolic supplement by metabolically engineered Escherichia coli. Metab. Eng. 2024, 84, 48–58. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhuang, M.; Song, J.; Hu, X.; Wang, X. Metabolic Engineering of Escherichia coli Nissle 1917 for Efficient Production of p-Coumaric Acid. ACS Synth. Biol. 2026, 15, 210–222. [Google Scholar] [CrossRef] [Scilit]
- Yu, Y.; Gong, B.; Wang, H.; Yang, G.; Zhou, X. Chromosome evolution of Escherichia coli Nissle 1917 for high-level production of heparosan. Biotechnol. Bioeng. 2023, 120, 1081–1096. [Google Scholar] [CrossRef] [Scilit]
- Hu, S.; Zhou, S.; Zheng, M.; Xiong, H.; Yin, G.; Yang, F.; Dong, P.; Chen, J.; Xu, R.; Kang, Z. Reprogramming the intrinsic capsular polysaccharide biosynthesis pathway for efficient secretory production of chondroitin in Escherichia coli Nissle 1917. Chem. Eng. J. 2026, 535, 175481. [Google Scholar] [CrossRef] [Scilit]
- Hu, M.; Zhang, T. Metabolic engineering of the probiotic Escherichia coli Nissle 1917 for lacto-N-triose II production. Food Biosci. 2024, 59, 103959. [Google Scholar] [CrossRef] [Scilit]
- Liu, D.; Ton, P.M.; Zong, D.; Zarrinpar, A.; Ding, Y. Expression of fluorescence reporters and natural products in native gut Escherichia coli. ACS Synth. Biol. 2025, 14, 1557–1566. [Google Scholar] [CrossRef] [Scilit]
- Wang, Z.; Dai, Y.; Azi, F.; Dong, M.; Xia, X. Deciphering the crucial roles of the quorum-sensing transcription factor SdiA in NADPH metabolism and (S)-equol production in Escherichia coli Nissle 1917. Antioxidants 2024, 13, 259. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Amiri-Jami, M.; Abdelhamid, A.G.; Hazaa, M.; Kakuda, Y.; Griffths, M.W. Recombinant production of omega-3 fatty acids by probiotic Escherichia coli Nissle 1917. FEMS Microbiol. Lett. 2015, 362, fnv166. [Google Scholar] [CrossRef] [Scilit]
- Li, R.; Wang, D.; Zhang, X.L.; Luo, J.M.; Dai, Z.B. Engineered probiotic Escherichia coli Nissle 1917 for controlled delivery of lycopene. Zhongguo Zhongyao Zazhi 2025, 50, 5733–5741. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Robinson, E.A.; Frankenberg-Dinkel, N.; Xue, F.; Wilks, A. Recombinant production of biliverdin IXβ and δ isomers in the T7 promoter compatible Escherichia coli Nissle. Front. Microbiol. 2021, 12, 787609. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fiege, K.; Frankenberg-Dinkel, N. Construction of a new T7 promoter compatible Escherichia coli Nissle 1917 strain for recombinant production of heme-dependent proteins. Microb. Cell Factories 2020, 19, 190. [Google Scholar] [CrossRef] [Scilit]
- Wu, H.; Wei, J.; Zhao, X.; Liu, Y.; Chen, Z.; Wei, K.; Lu, J.; Chen, W.; Jiang, M.; Li, S. Neuroprotective effects of an engineered Escherichia coli Nissle 1917 on Parkinson’s disease in mice by delivering GLP-1 and modulating gut microbiota. Bioeng. Transl. Med. 2023, 8, e10351. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Shao, F.; Wu, R.; Li, Z.-J. Enhanced heparosan biosynthesis in Escherichia coli Nissle 1917 through carbon flux redirection. J. Biosci. Bioeng. 2025, 140, 193–199. [Google Scholar] [CrossRef] [Scilit]
- Revelles, O.; Millard, P.; Nougayrède, J.P.; Dobrindt, U.; Oswald, E.; Létisse, F.; Portais, J.C. The Carbon Storage Regulator (Csr) System Exerts a Nutrient-Specific Control over Central Metabolism in Escherichia coli Strain Nissle 1917. PLoS ONE 2013, 8, e66386. [Google Scholar] [CrossRef] [Scilit]
- Chen, Y.; Wan, Z.; Li, Z.-J. Development of sucrose-utilizing Escherichia coli Nissle 1917 for efficient heparosan biosynthesis. Metabolites 2025, 15, 410. [Google Scholar] [CrossRef] [Scilit]
- Valdebenito, M.; Crumbliss, A.L.; Winkelmann, G.; Hantke, K. Environmental factors influence the production of enterobactin, salmochelin, aerobactin, and yersiniabactin in Escherichia coli strain Nissle 1917. Int. J. Med. Microbiol. 2006, 296, 513–520. [Google Scholar] [CrossRef] [Scilit]
- Effendi, S.S.W.; Toya, Y.; Shimizu, H.; Xue, C.; Ng, I.S. Utilizing Ribose 1,5-Bisphosphate Isomerase and RuBisCO-Equipped Escherichia coli Nissle for Low-Carbon Footprint GABA Production. ACS Sustain. Chem. Eng. 2024, 12, 11093–11098. [Google Scholar] [CrossRef] [Scilit]
- Liu, L.H.; Zhang, Z.; Xu, B.; Yang, G.; Cui, H.; Su, L.; Zhang, Y.; Sun, B.; Wu, Y.R.; Jiang, A. Directed evolution of Escherichia coli Nissle 1917 functioning as a methylotrophic chassis. Chem. Eng. J. 2025, 518, 164608. [Google Scholar] [CrossRef] [Scilit]
- Clare, C.; Rutter, J.W.; Fedorec, A.J.H.; Frank, S.; Barnes, C.P. Bacterial microcompartment utilization in the human commensal Escherichia coli Nissle 1917. J. Bacteriol. 2024, 206, e00269-24. [Google Scholar] [CrossRef] [Scilit]
- Millard, P.; Pérochon, J.; Létisse, F. Functional Analysis of Deoxyhexose Sugar Utilization in Escherichia coli Reveals Fermentative Metabolism under Aerobic Conditions. Appl. Environ. Microbiol. 2021, 87, e00719-21. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xu, B.; Liu, L.H.; Lai, S.; Chen, J.; Wu, S.; Lei, W.; Lin, H.; Zhang, Y.; Hu, Y.; He, J.; et al. Directed Evolution of Escherichia coli Nissle 1917 to Utilize Allulose as Sole Carbon Source. Small Methods 2024, 8, 2301385. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kaznadzey, A.D.; Rybina, A.A.; Bessonova, T.A.; Korshunov, D.S.; Tutukina, M.N.; Gelfand, M.S. Sulfoquinovose Catabolism in E. coli Strains: Compositional and Functional Divergence of yih Gene Cassettes. Int. J. Mol. Sci. 2025, 26, 10351. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sabri, S.; Nielsen, L.K.; Vickers, C.E. Molecular control of sucrose utilization in Escherichia coli W, an efficient sucrose-utilizing strain. Appl. Environ. Microbiol. 2013, 79, 478–487. [Google Scholar] [CrossRef] [Scilit]
- Datta, P.; Fu, L.; Brodfuerer, P.; Dordick, J.S.; Linhardt, R.J. High density fermentation of probiotic E. coli Nissle 1917 towards heparosan production, characterization, and modification. Appl. Microbiol. Biotechnol. 2021, 105, 1051–1062. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yu, D.; Zhu, L.; Ding, Y.-X.; Mao, L.-J.; Xiong, M.; Jin, X.-X.; Ma, Y.; Wang, F.-Q.; Xiong, L.-B. Engineering of endogenous plasmids in probiotic Escherichia coli Nissle 1917 for autonomous accumulation of 5-aminolevulinic acid. J. Biotechnol. 2025, 409, 157–164. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hu, M.; Zhang, T.; Miao, M.; Li, K.; Luan, Q.; Sun, G. Expectations for employing Escherichia coli Nissle 1917 in food science and nutrition. Crit. Rev. Food Sci. Nutr. 2025, 65, 1802–1810. [Google Scholar] [CrossRef] [Scilit]
- Aranda, M.; Arroba, J.; Naranjo, V.; Velástegui, M.; Telenchana, M.; Herrera, D. Potential of scientific and biotechnological applications of Escherichia coli Nissle 1917: Systematic review. Int. J. Drug Deliv. Technol. 2026, 16, 638–645. [Google Scholar] [CrossRef] [Scilit]
- Dong, M.-M.; Li, Y.-X.; Xu, M.; Ding, Y.-X.; Song, L.; Xiong, J.; Wei, D.-Z.; Xiong, L.-B.; Wang, F.-Q. An Escherichia coli Nissle 1917-based live therapeutics platform with integrated phage resistance and programmable temperature sensitivity. J. Control. Release 2025, 387, 114188. [Google Scholar] [CrossRef] [Scilit]
- Gurbatri, C.R.; Lia, I.; Vincent, R.; Coker, C.; Castro, S.; Treuting, P.M.; Hinchliffe, T.E.; Arpaia, N.; Danino, T. Engineered probiotics for local tumor delivery of checkpoint blockade nanobodies. Sci. Transl. Med. 2020, 12, eaax0876. [Google Scholar] [CrossRef] [Scilit] [PubMed]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.