


Simple Summary
The Qinghai–Tibetan Plateau is covered by vast alpine grasslands that are vital to local livestock farming. This study explores how changes in altitude and soil depth affect plant nutrient content, soil properties, and the tiny organisms living in the soil. Aboveground biomass declined from low to high altitude, and crude protein from 12.8% to 10.1% along the altitude gradient. Soil pH ranged from 7.6 to 6.4 across altitude and soil-depth groups. Ammonium nitrogen content was significantly higher at high altitude in the 20–30 cm layer compared with low- and mid-altitude soils (p < 0.05). Microbial community composition, predicted functional potentials, and co-occurrence network properties differed across altitude and soil-depth groups. These findings demonstrate that spatial variations in altitude and soil depth are associated with forage quality, soil conditions, and microbial community patterns in alpine grasslands.
Abstract
Altitude and soil depth were associated with vegetation, soil properties, and microbial communities in alpine ecosystems, yet a comprehensive understanding of how these gradients shape soil microbial and physicochemical characteristics on the Qinghai–Tibetan Plateau remains limited. Along altitudinal gradients (low, mid, and high) and soil depths (0–10 cm, 10–20 cm, 20–30 cm), we systematically investigated vegetation traits, soil physicochemical properties, microbial community composition, functional pathways, and co-occurrence networks. Aboveground biomass, community-weighted height, and soil pH declined with altitude. Soil pH and ammonium nitrogen were significantly associated with bacterial community variation in the RDA analyses. Surface and deeper soil layers differed in bacterial taxonomic composition and predicted functional potentials. Co-occurrence network properties also varied across altitude and soil-depth groups. These findings describe spatial associations among vegetation, soil conditions, and bacterial community patterns during the sampling period. This study improves our understanding of how interacting environmental structure soil microbial communities and influence ecosystem functioning in alpine ecosystems.
1. Introduction
Soil microorganisms are fundamental regulators of terrestrial ecosystem functioning, mediating organic matter decomposition, carbon sequestration, and nutrient cycling processes that determine ecosystem productivity and stability [1]. Through diverse metabolic strategies, microorganisms regulate the transformation and availability of carbon and nitrogen resources, thereby controlling the feedback between soil processes and vegetation dynamics, which are the main driving forces of soil ecosystems [2]. However, microbial communities are not randomly assembled; instead, their composition and functional potential are shaped by environmental filtering, resource availability, and interactions with vegetation. Consequently, understanding how microbial communities respond to environmental gradients is essential for predicting ecosystem responses to global environmental changes.
Altitude gradients provide natural environmental experiments for exploring microbial adaptation because they integrate multiple ecological drivers, including temperature, precipitation, ultraviolet radiation, vegetation productivity, and soil nutrient availability [3]. Along increasing elevations, declining temperature and altered moisture regimes can modify plant productivity, litter input, and soil physicochemical properties, thereby influencing microbial community assembly and ecological functioning. Previous studies have demonstrated that soil pH, soil organic carbon (SOC), and nitrogen availability are major environmental factors regulating microbial diversity and composition across mountain ecosystems [4,5]. However, altitude-associated environmental changes are often accompanied by alterations in vegetation composition and productivity, making it difficult to distinguish the direct effects of climatic filtering from plant-mediated effects on soil microbial communities.
In addition to horizontal environmental gradients, soil depth represents an important vertical ecological gradient that may strongly contribute to microbial habitat conditions. Surface soils receive continuous inputs of plant-derived carbon through litter decomposition and root exudation, providing abundant resources for copiotrophic microorganisms. In contrast, deeper soil layers generally experience reduced carbon availability, lower oxygen diffusion, and stronger nutrient limitation, favoring microorganisms with oligotrophic strategies and specialized metabolic capacities [6]. Although vertical differentiation of microbial communities has been reported in forest and peatland ecosystems [7,8], most studies have examined either elevational variation or soil depth effects independently.
Vegetation represents another critical component linking environmental gradients with belowground microbial processes [9]. Changes in altitude can alter plant community composition, biomass production, and nutrient inputs, which subsequently influence microbial habitats and biogeochemical processes. For example, alpine meadow vegetation on the Qinghai–Tibetan Plateau (QTP) exhibits strong spatial differentiation along environmental gradients, with variations in dominant species, aboveground biomass (AGB), and plant nutrient characteristics [9,10]. Conversely, microbial-mediated nutrient transformations can regulate plant productivity and vegetation characteristics, forming complex plant–soil–microbe feedbacks [11,12]. However, the contribution of vegetation variation to microbial community assembly across combined altitude and soil depth gradients remains poorly understood.
The QTP represents one of the most environmentally sensitive terrestrial ecosystems, where alpine ecosystems are strongly influenced by climatic gradients and soil heterogeneity. Although previous studies have investigated altitude-associated changes in vegetation, soil properties, and microbial communities across the QTP, the mechanisms underlying the coupled regulation of microbial communities by elevational environmental filtering, vertical soil heterogeneity, and vegetation variation remain unclear. Based on this framework, we hypothesized that (1) bacterial community composition differs among altitudes and soil depths, with altitude-related differences depending on soil depth; (2) variation in bacterial community composition is associated with soil pH, SOC, mineral nitrogen availability, and vegetation characteristics, including AGB and forage nutrient content; and (3) surface soils are relatively enriched in bacterial taxa associated with copiotrophic strategies, whereas deeper soils are relatively enriched in taxa associated with oligotrophic strategies. To evaluate these hypotheses, we selected three alpine regions at low, middle, and high altitudes with similar vegetation types, climatic zones, and soil categories to minimize non-altitude-related variability. We collected forage samples and soil samples from three depths (0–10, 10–20, and 20–30 cm). Our objectives were to examine the effects of altitude and soil depth on soil physicochemical properties and bacterial community composition and identify soil and vegetation variables associated with bacterial community variation.
2. Materials and Methods
2.1. Study Area and Sample Collection
The study was conducted in August 2023 in Gannan Tibetan Autonomous Prefecture, located on the northeastern margin of the Qinghai–Tibetan Plateau (QTP), Gansu Province, China. This region represents a typical alpine ecosystem characterized by strong environmental gradients associated with altitude changes. Three altitude zones were selected: low (3000–3100 m), middle (3300–3400 m), and high altitude (3500–3600 m). At each altitude, vegetation characteristics were surveyed in 12 spatially separated 1 m × 1 m quadrats (n = 12 per altitude; 36 quadrats in total). Nine of these quadrats at each altitude were also used for soil sampling. At each soil sampling quadrat, soil cores were collected from five positions using a 5 cm diameter soil corer and separated into three soil depths (0–10, 10–20, and 20–30 cm) [13]. The five cores collected from the same quadrat and depth were thoroughly homogenized to form one composite soil sample. We collected 81 composite soil samples in total (3 altitudes × 9 sampling points × 3 soil depths). Each composite sample was divided into two portions: one was used for bacterial 16S rRNA gene sequencing, and the other was used to determine soil physicochemical properties.
The dominant species at low altitude were Elymus nutans Griseb, Kobresia pygmaea (C.B.Clarke) C.B.Clarke and Medicago falcata L., the dominant species at mid-altitude were Kobresia pygmaea, Elymus nutans, and the dominant species at high altitude were Potentilla anserina L., Kobresia pygmaea, Elymus nutans and Anaphalis lactea Maxim. Plant species identity, richness, density, and species-specific height were recorded in each vegetation quadrat. Within each quadrat, vegetation from a 0.5 m × 0.5 m area was clipped at ground level using hand shears and placed in paper envelopes for aboveground biomass (AGB) determination. Sample groups were designated according to altitude and soil depth. L1, L2, and L3 represent soil depths of 0–10 cm, 10–20 cm, and 20–30 cm in low altitudes; M1, M2, and M3 represent soil depths of 0–10 cm, 10–20 cm, and 20–30 cm in middle altitudes; and H1, H2, and H3 represent soil depths of 0–10 cm, 10–20 cm, and 20–30 cm in high altitudes.
2.2. Determination of Plant Nutrient Contents
The grass samples were dried for 48 h at 65 °C, weighed using a digital balance, and the AGB (g·m−2) was calculated by dividing the dry weight of the grass sample with the sampling area (0.25 m2). Thereafter, the dried grass samples were ground through a 1 mm screen for chemical composition determination. The dry matter, crude ash, neutral detergent fiber, acid detergent fiber and ether extract were determined according to the official methods of the Association of Official Analytical Chemists (AOAC International) [14]. Total nitrogen was analyzed using flash combustion and thermal conductivity detection (Model 1500, Carlo Erba Instruments, Milan, Italy), and crude protein content was calculated as N × 6.25 crude protein [14].
2.3. Measurement of Soil Physicochemical Properties
Soil physicochemical properties, including pH, electric conductivity, SOC, soil NH4+-N and nitrate (NO3−-N) were determined. For pH and electric conductivity measurement, 1 g of each soil sample was extracted with 5 mL distilled water, and the pH and electric conductivity of soil samples were measured in the supernatant using a Hach pH meter (Hach Company, Loveland, CO, USA) and an electrical conductivity (EC) meter (DDSJ-319L, Shanghai, China), respectively. The SOC was determined by the oil bath K2CrO7 titration method [15]. For NH4+-N and NO3−-N determination, fresh soil samples were extracted with KCl and then measured on an UV spectrophotometer (UV-2450, Shimadzu Corporation, Kyoto, Japan) according to the method of Ren et al. [16].
2.4. 16S rRNA Gene Sequencing and Data Analysis
Total genomic DNA from samples was extracted using the CTAB (Cetyltrimethylammonium Bromide) method [17]. The concentration and purity of the extracted DNA were monitored using a NanoDrop spectrophotometer (ND-2000; NanoDrop Technologies Inc., Wilmington, DE, USA) and 1% agarose gel, and then the concentration of DNA of each sample was diluted to 10 ng/µL using sterile water. The V3-V4 regions of 16S rRNA genes were amplified with specific primers 341F (5′-CCTAYGGGRBGCASCAG-3′) and 806R (5′-GGACTACNNGGGTATCTAAT-3′). All the PCR reactions were performed as described in the literature [18]. PCR products were mixed in equimolar proportions and then purified with a Gel Extraction Kit (Qiagen, Hilden, Germany). Sequencing libraries were generated using NEB Next® Ultra DNA Library Prep Kit for Illumina (New England Biolabs, Ipswich, MA, USA), with index codes added following the manufacturer’s recommendations. Library quality was assessed on an Agilent 5400 Bioanalyzer (Agilent Technologies, Santa Clara, CA, USA). Thereafter, the library was sequenced on an Illumina NovaSeq platform (Illumina, San Diego, CA, USA) at Wekemo Tech Group (Shenzhen, China) and 250 bp paired-end reads were generated.
Raw paired-end reads were imported into QIIME 2 (version 2022.2) and processed using its DADA2 workflow (DADA2 version 1.22.0) [19,20]. Forward and reverse reads were trimmed by 23 and 26 bp, respectively, and truncated at 249 bp. Reads with expected errors >2 was filtered. Denoising was performed independently for each sample, using 1,000,000 reads to train the error model. Paired-end reads were merged with a minimum overlap of 12 bp, and chimeras were removed using the consensus method. The workflow generated an amplicon sequence variants (ASVs) abundance table and representative sequences. Taxonomy was assigned using the QIIME 2 q2-feature-classifier plugin and the SILVA 16S rRNA reference database (release 138.2) [21,22]. Sequences assigned to mitochondria and chloroplasts were removed before downstream analyses.
The ASVs count table was rarefied to 50,966 sequences per sample, the minimum sequencing depth after processing; all 81 samples were retained. Chao1 richness, Shannon diversity, and Simpson diversity were calculated from the rarefied ASVs table. Beta-diversity was assessed using Bray–Curtis, weighted UniFrac, and unweighted UniFrac distance matrices, followed by principal coordinate analysis and nonmetric multidimensional scaling [23,24]. Functional Annotation of Prokaryotic Taxa (FAPROTAX, v1.2.6) was used to infer predicted functional potentials from ASV taxonomic assignments and abundances [25]. Functional results are described as predicted functional potentials inferred from 16S rRNA gene data rather than directly measured microbial activities.
2.5. Co-Occurrence Network Analysis
Microbial co-occurrence networks were constructed separately for each altitude × soil depth combination, including low-, mid-, and high-altitude soils at 0–10, 10–20, and 20–30 cm, resulting in nine networks in R (v4.3). Networks were constructed at the ASV level. To reduce the influence of rare taxa, ASVs with a cumulative relative abundance >0.05% across the samples within each altitude × soil depth group were retained. Pairwise Spearman’s rank correlations were calculated among retained ASVs, and p values were adjusted for multiple comparisons using the false discovery rate (FDR) procedure [26]. Associations were defined as significant at |r| > 0.85 and adjusted p < 0.05. An undirected co-occurrence network was then constructed using the igraph package (v2.2.1) in R. Network topology was characterized by calculating the number of nodes and edges, average degree, clustering coefficient, mean path length, and modularity, which together describe the structural properties of microbial networks. Network visualization was performed using Gephi (v0.10.1), with edges colored by correlation type and nodes colored by phylum-level taxonomy.
2.6. Statistical Analysis
The CWH was calculated on the basis of mean plant height and the percent aboveground net primary production of each plant species in the community according to Quan et al. [27]. On the basis of the mean plant height and the percentage of abundance in the community, the CWH was calculated as:
where Pi is the percent abundance of community i, Hi is the mean plant height of community i, and S is the number of communities [28].
CWH = iSPi × Hi
Prior to statistical analyses, the normality of data distribution was assessed using the Shapiro–Wilk test, and homogeneity of variances was evaluated using Levene’s test. Considering the hierarchical structure of the sampling design, each sampling site was considered as the independent experimental unit. One-way ANOVA, followed by Tukey’s honestly significant difference (HSD) test, was used to compare differences in soil physicochemical properties, plant species richness, density, above-ground biomass (AGB), and community-weighted mean height (CWH) and the relative abundance of microbiota among sampling sites. Two-way ANOVA was performed to evaluate the effects of altitude-associated gradients, soil depth, and their interaction on soil physicochemical properties and microbial abundance. Mantel tests assessed statistical associations between individual microbial α-diversity indices and individual vegetation characteristics. For each altitude, the analysis included the nine soil sampling quadrats and their nine spatially matched vegetation observations (n = 9). Euclidean distance matrices were calculated separately for Chao1 richness, Shannon diversity, Simpson diversity, and each vegetation variable. All statistical analyses were performed using SPSS Statistics (Version 26.0; IBM Corp., Armonk, NY, USA), with statistical significance defined as p < 0.05.
3. Results
3.1. Vegetation, Soil Characteristics Along Altitudinal Gradients and Soil Depths
The species richness and density were not different (p > 0.05) among the three altitudes, whereas greater (p < 0.05) AGB and CWH were observed at low-altitude than at mid- and high-altitude alpine ecosystems (Table 1). The contents of dry matter, crude fat, neutral detergent fiber and crude ash of the forage samples did not differ along the altitudes; however, the crude protein at high altitude was significantly lower (p < 0.05) than that at low altitude. Meanwhile, the acid detergent fiber at mid-altitude was higher (p < 0.05) than that at low and high altitudes; it did not differ between low and high altitudes. Regression analysis showed that the AGB (R2 = 0.21303, p = 0.0027) and CWH (R2 = 0.31685, p < 0.001) were negatively correlated with altitude (Figure S1).
Table 1.
Vegetation characteristics and nutrient contents of natural pastures along altitude of Gannan alpine ecosystems located at the northeastern edge of Gannan alpine ecosystems.
Effects of altitude, soil depth and their interaction on soil physicochemical properties (including pH, SOC, NH4+-N, NO3−-N and EC) were analyzed, and there was an altitude × depth interaction (p < 0.05) for all of these indices (Table 2 and Table S1). The pH of the soil decreased (p < 0.05) as either the altitude or depth increased, with significantly lower pH at the 20–30 cm layer than at the 0–10 cm layer at the same altitude and significantly lower pH at higher altitude at each soil layer. The SOC at middle and high altitudes was greater (p < 0.05) than that at low altitude, while at each altitude, the SOC was almost not affected by soil depth at middle or high altitude. Significantly greater (p < 0.05) NH4+-N contents were observed at high altitude than at low and mid-altitude. NH4+-N contents in surface soil (0–10 cm) were higher (p < 0.05) than in deeper layers (20–30 cm) at low and mid-altitude, whereas the NH4+-N contents significantly increased (p < 0.05) with increasing soil layer at high altitude. Greater (p < 0.05) NO3−-N contents were detected at surface-layer soil of middle and high altitudes and in medium-layer soil at high altitude, but there was no difference (p > 0.05) among the deeper-layer samples (20–30 cm). At low altitude, the soil EC was significantly higher in the surface layer than in deeper layers; meanwhile, the EC in the surface soil at low altitude was significantly higher than that in mid- and high-altitude soil.
Table 2.
Effects of altitudes and soil depths on physicochemical properties of soil collected from Gannan alpine ecosystems.
3.2. Soil Microbial Communities Along Altitudinal Gradients
3.2.1. Summary of Collective Sequencing Data of Soil Microbiota
A total number of 8,740,234 raw reads were generated from 81 soil samples. After data processing, including filtering, quality control, assembling of paired-end reads, and removal of primers, chimeras, and low-confidence singletons, a total of 7,957,816 high-quality reads, with a high-quality sequence ratio of 91.1%, were used for data analysis. A total of 67,705 ASVs were identified by the analysis based on 97% nucleotide sequence identity among reads. There were 778 shared bacterial ASVs among different soil depths and altitudes; however, a great number of individual ASVs were observed in each soil layer among different altitudes (Figure S2). Further, principal component analysis (PCA) based on 16S rRNA amplicon sequence variants revealed variation in microbial community structure among different altitude groups. In several comparisons, samples showed partial separation along PC1 and PC2, indicating altitude-associated shifts in community composition, although some overlap among groups was observed (Figure S3). Effects of altitude, soil depth and their interaction on the α-diversity indices (including Chao 1, Shannon, and Simpson) of soil microbiota were analyzed, and no altitude × depth interactions were observed (Table S2). At low and high altitudes, different patterns for the Chao 1 index were observed. It increased (p < 0.05) with soil depth at low altitude, but it decreased with soil depth at high altitude; meanwhile, it significantly increased (p < 0.05) with altitude at the surface soil. The Shannon and Simpson indexes remained stable at different soil depths and altitudes.
Taxonomic composition of the soil bacteria by altitude and depth was compared on the basis of percentage mean relative abundance. Except for some unclassified phyla, Proteobacteria (average 21.5%) and Acidobacteria (average 20.8%) were the dominant phyla, followed by Actinobacteriota, Methylomirabilota and Chloroflexota. Similarly, UBA12499 and VBCG01 were the dominant genera after the identification of the top 10 species at the genus level.
3.2.2. Differential Microbes
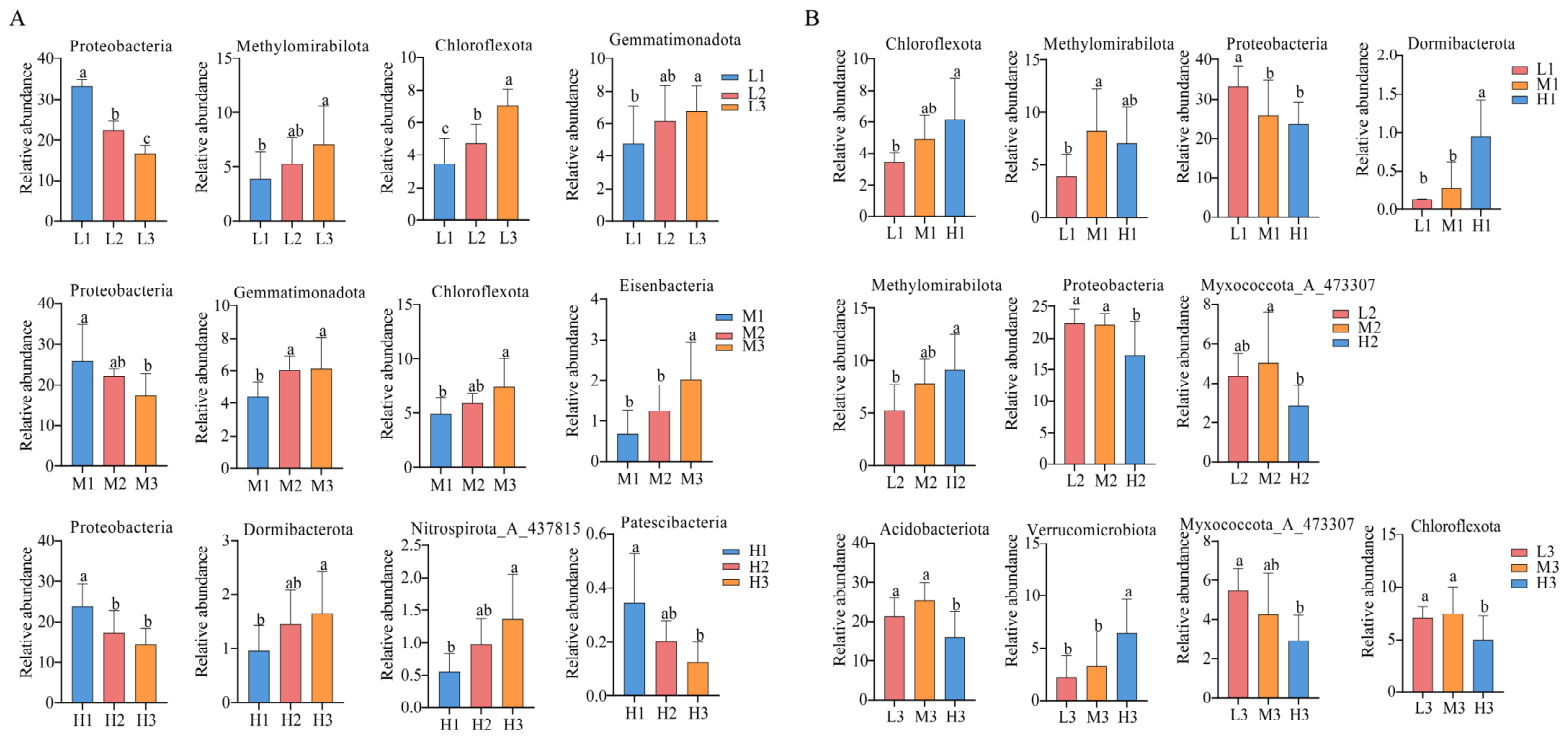
The relative abundances of microbes at different soil depth of each altitude were compared, and differential microbes identified are shown in Figure 1A. Proteobacteria was the most dominant phylum at low-, mid- and high-altitudes, with its relative abundance significantly decreased (p < 0.05) as the soil depths increased at all the three altitudes. At low altitude, the relative abundance of Methylomirabilota was higher (p < 0.05) in the deeper layer (L3) than the surface layer (L1), and Desulfobacterota_B was higher (p < 0.05) in L3 and L2 than L1. In addition, the relative abundance of Nitrospirota_A_437815 was highest (p < 0.05) in L3, followed by L2 and L1 (p < 0.05). At middle altitude, the relative abundances of Chloroflexota, Gemmatimonadota and Eisenbacteria increased as the soil depth increased, with significantly greater (p < 0.05) abundance in M3 than in M1. At high altitude, the relative abundances of Nitrospirota_A_437815 and Dormibacterota were higher in the deeper layer (H3) than in the surface layer (H1); in contrast, Patescibacteria was higher (p < 0.05) in the surface layer (H1) than in the deeper layer (H3). At the genus level, the relative abundance of VBCG01 was higher (p < 0.05) in the surface layer (L1, M1) than in the deeper layer (L3, M3), and Usitatibacter was higher (p < 0.05) in L1 and L2 than L3, and higher (p < 0.05) in H1 than H3 (Figure S4A).
Figure 1.
Differential soil microbes at the phylum level along soil depths (A) and altitudinal gradients (B) in alpine grasslands of Gannan prefecture. L1, L2, and L3 represent soil depths of 0–10 cm, 10–20 cm, and 20–30 cm in low altitudes; M1, M2, and M3 represent soil depths of 0–10 cm, 10–20 cm, and 20–30 cm in middle altitudes; and H1, H2, and H3 represent soil depths of 0–10 cm, 10–20 cm, and 20–30 cm in high altitudes. The same applies below. Different lowercase letters represent significant differences with p < 0.05.
3.2.3. Metabolic Pathways
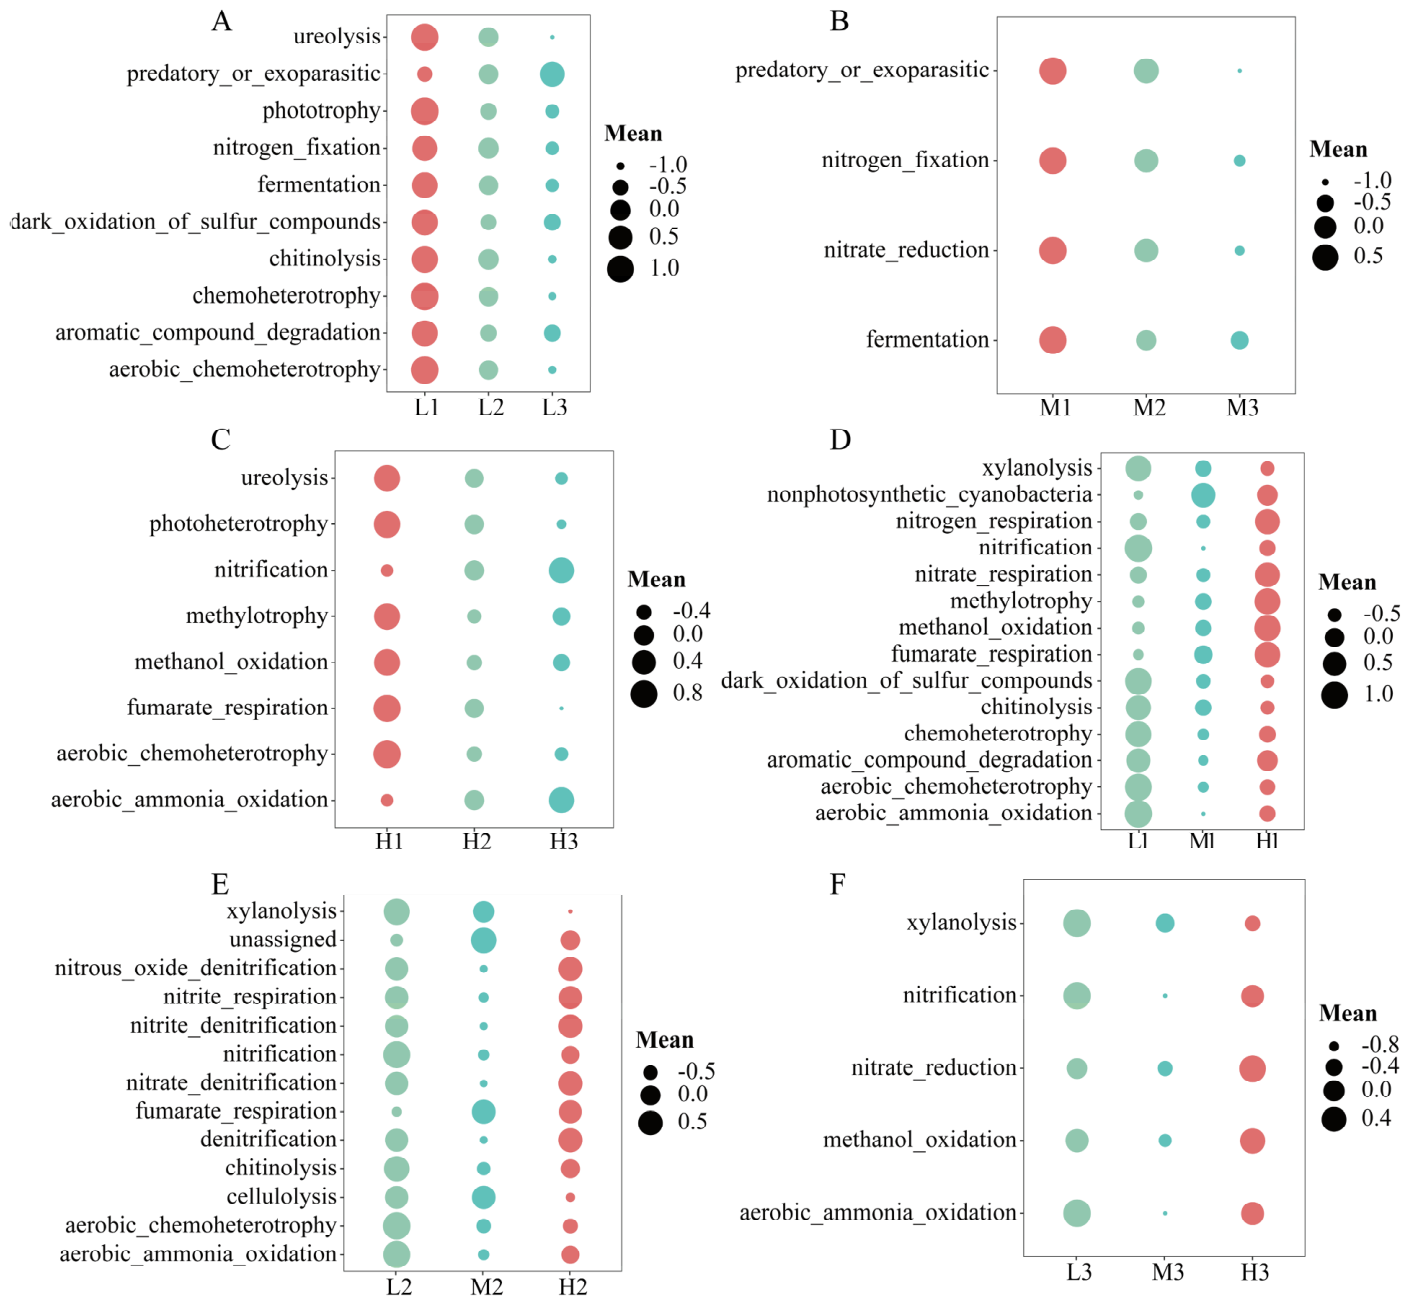
Based on FAPROTAX-predicted functional potentials, most soil microbial functions (including ureolysis, phototrophy, nitrogen fixation, fermentation, dark oxidation of sulfur compounds, chitinolysis, chemoheterotrophy, aromatic compound degradation and aerobic chemoheterotrophy) were higher (p < 0.05) in L1 than L2 or L3, but predatory or exoparasitic activity was lower (p < 0.05) in L1 than L3 (Figure 2). The enrichment function at mid-altitude was similar, with the four metabolic pathways in M1 higher (p < 0.05) than that in M3. At high altitude, nitrification and aerobic ammonia oxidation in H3 were higher (p < 0.05) than those in H1 (p < 0.05).
Figure 2.
Differences in soil microbial function prediction at metabolic pathways. (A–C) represent the comparison of microbial metabolic pathways among different soil depths of the same altitude (low, middle and high altitude, respectively); (D–F) represent the comparison of microbial metabolic pathways at the same soil depth but different altitudes.
3.3. Soil Microbial Communities in Different Soil Depths
3.3.1. Differential Microbes
The relative abundances of microbes at the same soil depth (0–10 cm, 10–20 cm, and 20–30 cm, respectively) but different altitudes were compared, with different microbes identified (Figure 1B). In surface soil (0–10 cm), the relative abundances of Chloroflexota and Dormibacterota were significantly higher at high altitude than at low or mid-altitude; whereas the Methylomirabilota and Nitrospirota-A-437815 had the highest abundance at mid-altitude. In the medium soil (10–20 cm), the relative abundances of Methylomirabilota and Dormibacterota were higher (p < 0.05) at high versus low altitude; while the relative abundances of Myxococota_A_473307 and Nitrospirota_A_437815 were greater at mid-altitude. In the deeper layer (20–30 cm), the relative abundance of Acidobacteriota was higher (p < 0.05) at low or mid-altitude than at high altitude; Eisenbacteria had the highest abundance at low altitude, and Verrucomicrobiota had the highest abundance at high altitude. At the genus level, the relative abundance of TA_21 was higher (p < 0.05) at low altitude than middle and high altitude in both the surface and the medium soil depths. In the medium soil depth, the relative abundances of UBA12499 and GWA2_73_35 increased with increasing altitude; VBCG01 was higher (p < 0.05) in M2 than L2. In deeper soil, the relative abundances of VBCG01, PSRF01, GWC2_73_18 and UBA11740 were higher at mid-altitude (Figure S4B).
3.3.2. Metabolic Pathways
At 0~10 cm, soil microbial function, including xylanolysis, nitrification, dark oxidation of sulfur compounds, chitinolysis, chemoheterotrophy, aromatic compound degradation, aerobic chemoheterotrophy, and aerobic ammonia oxidation, was higher (p < 0.05) in L1 than M1 or H1, whereas nitrogen respiration, nitrate respiration, methylothrophy, methanol oxidation, and fumarate respiration were higher in H1 (p < 0.05) than L1. At 10–20 cm, nitrification, aerobic chemoheterotrophy and aerobic ammonium oxidation were higher (p < 0.05) in L2 than in M2 or H2. At 20–30 cm, the predominant metabolic pathways were enriched in xylanosis, nitrification, nitrate reduction, methanol oxidation and aerobic ammonia oxidation, with comparable abundances between L3 and H3 (Figure 2).
3.4. Associations Between Soil Properties, Vegetation Characteristics, and Microbial Communities
3.4.1. Relationship Between the Soil Microbial Community, Soil Physicochemical Properties and Vegetation Characteristics
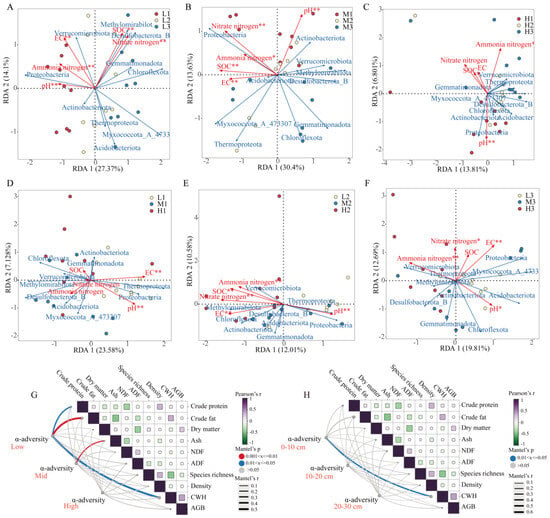
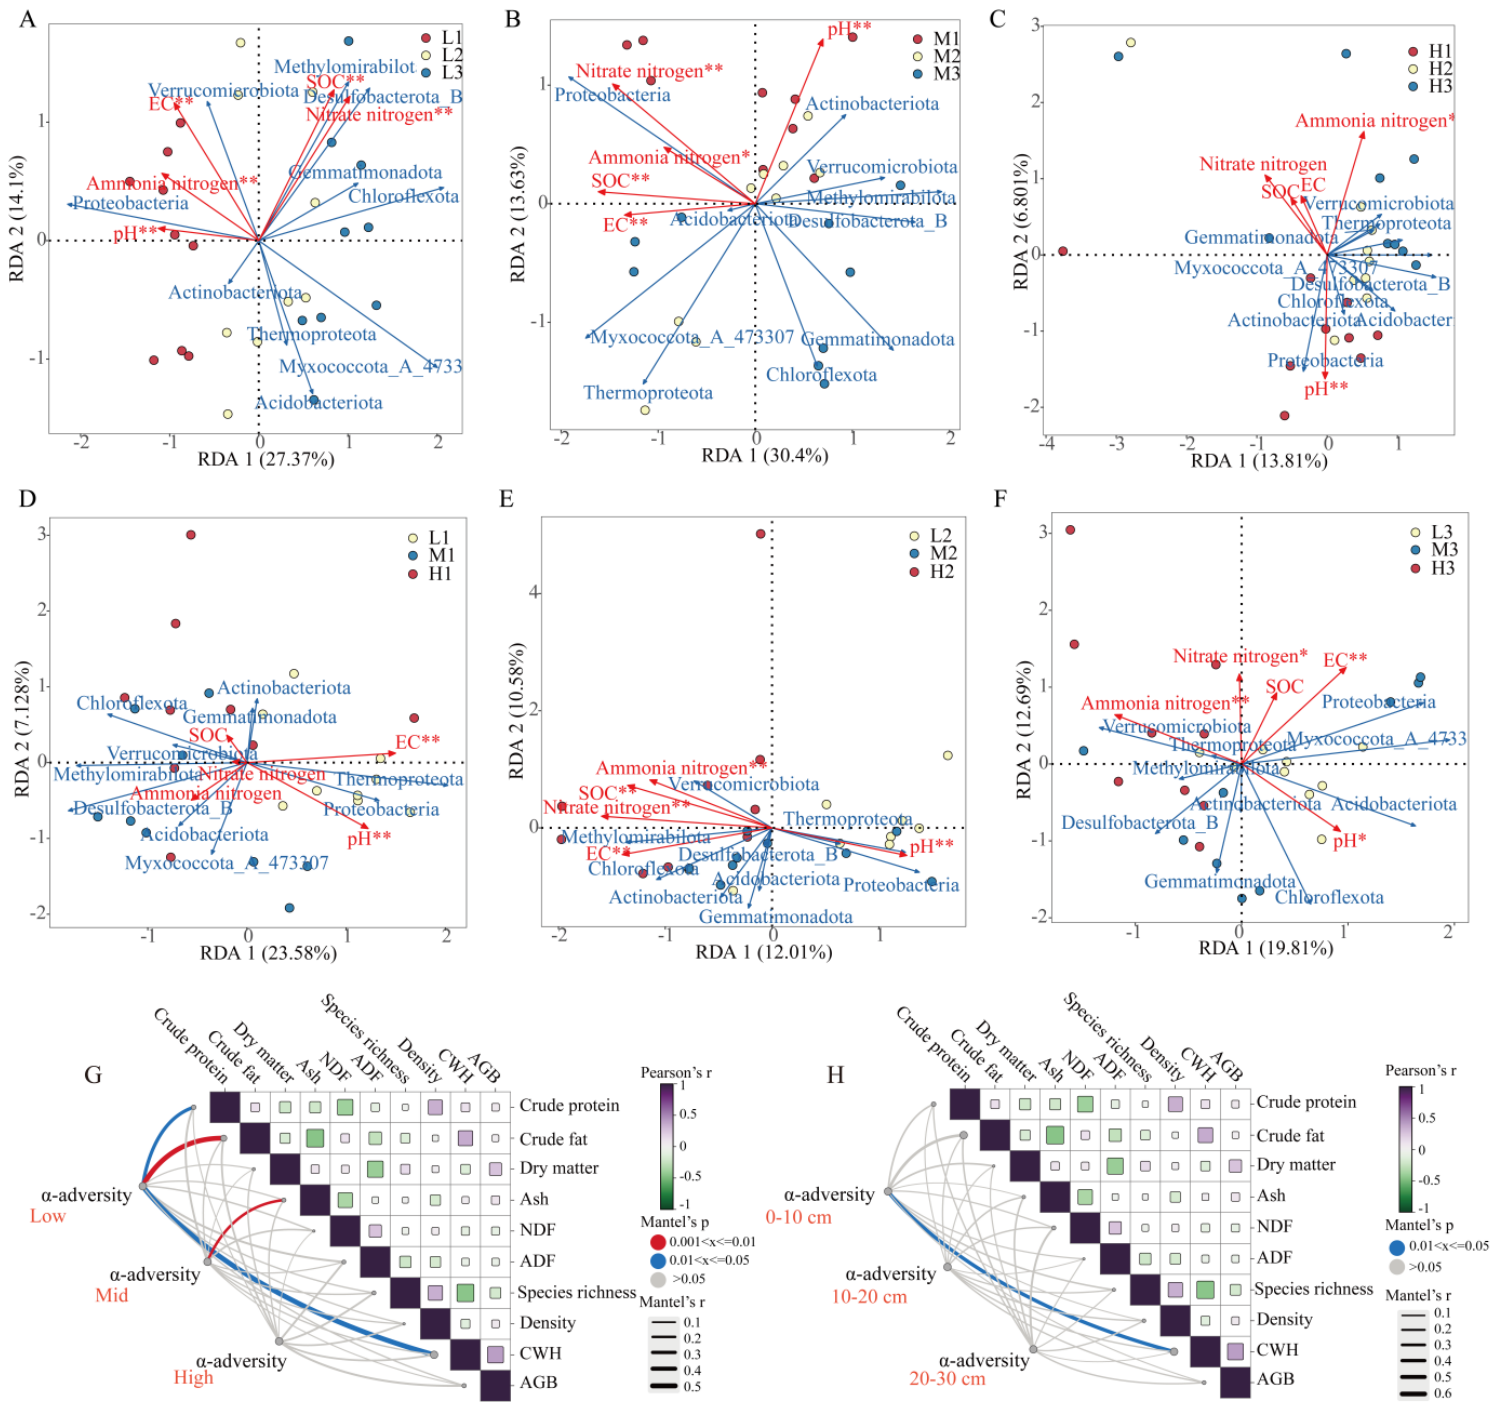
RDA analysis indicated that the associations between soil microbial community composition and soil physicochemical properties varied across altitudes (Figure 3A–C; Table S3). At low altitude, RDA1 and RDA2 explained 27.4% and 14.1% of the variation, respectively, yielding a cumulative explained proportion of 41.5% (Figure 3A). The overall model was significant (F = 3.961, p = 0.001), explaining 48.5% of the total variance (adjusted R2 = 0.363). At mid-altitude, the corresponding percentages were 30.4% and 13.6%, with a cumulative explained proportion of 44.0% (Figure 3B). The overall model explained 47.7% of the total variance (F = 3.826, p = 0.001; adjusted R2 = 0.352). At both altitudes, soil pH, SOC, EC, NH4+-N, and NO3−-N (p < 0.05) indicated significant associations with microbial community. In contrast, at high altitude, the first two axes jointly explained 20.6% of the total variance, whereas the overall model explained 26.2% and was not significant (F = 1.493, p = 0.104; adjusted R2 = 0.087). At low altitude, Mantel analysis indicated significant associations between the microbial community dissimilarity matrix and crude protein (Mantel r = 0.312, p = 0.014), crude fat (Mantel r = 0.493, p = 0.007), and community-weighted height (CWH; Mantel r = 0.505, p = 0.017) (Figure 3D). Among these variables, CWH showed the strongest association.
Figure 3.
Correlation between soil microbes, soil physicochemical properties and vegetation characteristics analyzed using redundancy and Mantel analysis. Redundancy analysis (RDA) between soil microbiota and soil physicochemical properties in different soil depths at low (A), middle (B), and high altitude (C) and at the 0–10 cm (D), 10–20 cm (E), and 20–30 cm (F) soil depths of these three altitudes. *, 0.01 < p < 0.05; **, p ≤ 0.01. Correlation between α-diversity of soil microbiota and vegetation characteristics at different altitudes (G) and soil depths (H) based on Mantel test. SOC, soil organic carbon; EC, electrical conductivity; NDF, neutral detergent fiber; ADF, acid detergent fiber; CP, crude protein; AGB, aboveground biomass; CWH, community-weighted height. Percentages shown on the RDA axes indicate the proportion of total variance explained by each axis. Overall model statistics and permutation test results are provided in Table S3.
Along the soil depth gradient, the associations between soil physicochemical properties and microbial communities varied among soil layers (Figure 3E–G). The first two RDA axes jointly explained 30.7% of the total variation, and the overall model explained 39.1% (F = 2.696, p = 0.001; adjusted R2 = 0.246) on the surface layer (0–10 cm), with pH and EC showing significant associations. In the 10–20 cm layer, the first two axes jointly explained 22.6% of the variance, and the overall model explained 32.9% (F = 2.058, p = 0.003; adjusted R2 = 0.169). In the 20–30 cm layer, these proportions were 32.5% and 41.3%, respectively (F = 2.951, p = 0.001; adjusted R2 = 0.273). Significant associations with pH and NH4+-N were observed in the 10–20 cm layer and 20–30 cm layer (p < 0.05). pH was positively correlated with the relative abundance of Proteobacteria but negatively correlated with that of Verrucomicrobiota across all the three soil layers. At the 0–10 cm soil layer, Mantel analysis indicated a significant association between the microbial community dissimilarity matrix and community-weighted height (CWH; Mantel r = 0.426, p = 0.036) (Figure 3H).
3.4.2. Soil Microbiota Co-Occurrence Patterns Along Altitudinal Gradients and Depths
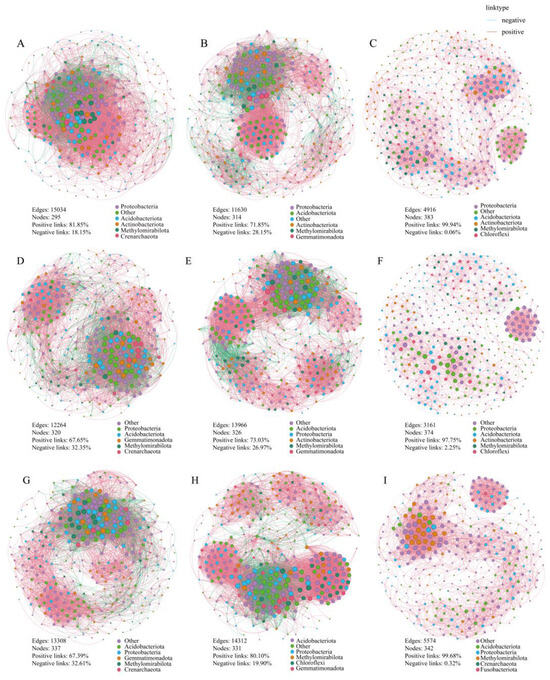
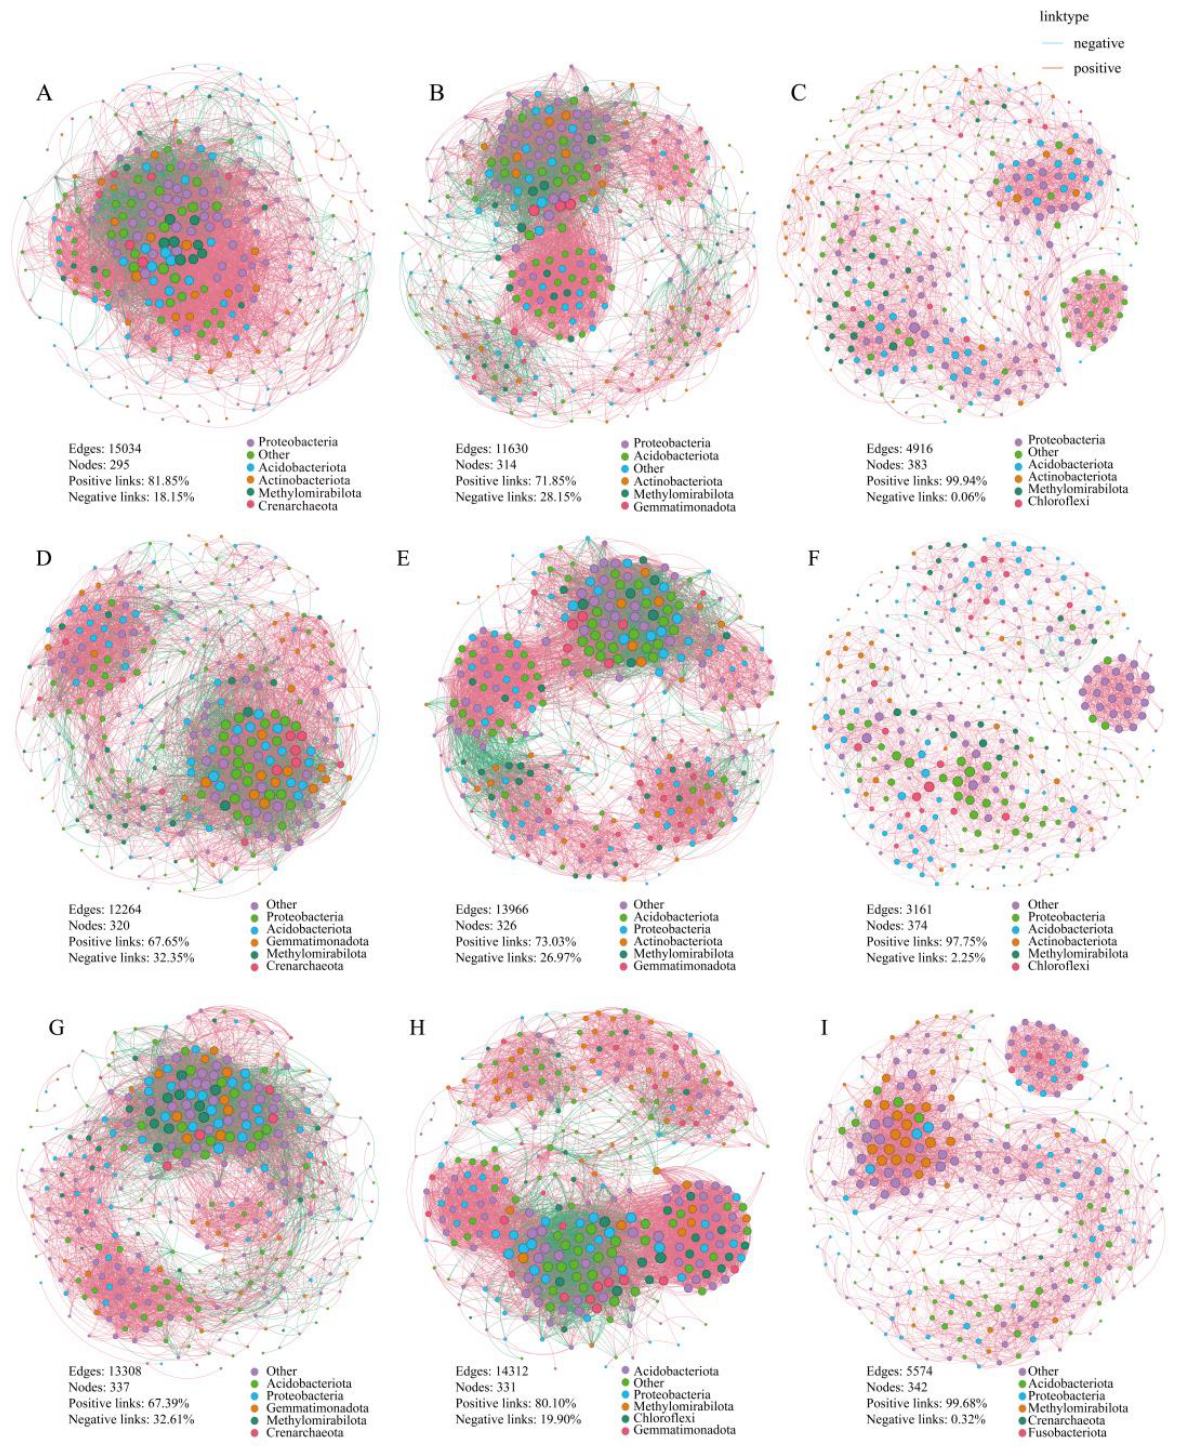
ASV-level co-occurrence networks, with nodes colored according to their phylum-level taxonomic affiliations, showed different topological properties among altitude × soil-depth groups (Figure 4; Table S4). At the phylum level, the soil microbial coexistence networks across all the altitude gradients exhibited significant depth-dependent changes (Figure 4). At low altitude (Figure 4A–C), despite an increase in the number of nodes, network connectivity decreased sharply with an increasing soil depth, as evidenced by a significant reduction in the number of edges, from 15,034 in the 0–10 cm layer to 11,630 in the 10–20 cm layer, and then to 4916 in the 20–30 cm layer. Similar depth-dependent simplification phenomena were also observed at mid-altitude (Figure 4D–F) and high-altitude (Figure 4G–I) regions, where the number of edges decreased from 12,264 and 13,308 in the surface and subsurface layers to 3161 and 5574 in the deeper layer. The proportion of positive connections increased with depth at low-altitude areas (from 81.9% to 99.9%), mid-altitude areas (from 67.7% to 97.8%) and high-altitude areas (from 67.4% to 99.7%).
Figure 4.
ASV-level soil microbial co-occurrence networks across altitude and soil-depth gradients. (A–C) represent the co-occurrence networks at 0–10, 10–20, and 20–30 cm layers of low altitude; (D–F) represent those at mid-altitude, while (G–I) represent those at high altitude. The nodes are colored by phylum level, and the size of each node is proportional to its degree. The line between each pair of nodes represents either positive (red) or negative (green) correlation with p < 0.05 and |r| > 0.85.
Along the altitude gradient, the coexistence network structure within the same soil layer exhibited significant changes in interaction patterns. In the surface layer (0–10 cm), the proportion of positive correlations continued to decrease with increasing altitude, from 81.85% at low altitude to 67.7% at mid-altitude and 67.3% at high altitude; whereas the proportion of negative correlations increased accordingly. In the 10–20 cm soil layer, the proportion of positive and negative correlations was reversed. The proportion of negative correlations was lowest in the 20–30 cm soil layer (Figure 4; Table S4). High-altitude networks also exhibited lower average clustering coefficients and higher modularity than the corresponding low- and mid-altitude networks at each soil depth (Table S4).
4. Discussion
4.1. Altitude-Associated Environmental Gradients Shape Vegetation and Soil Properties
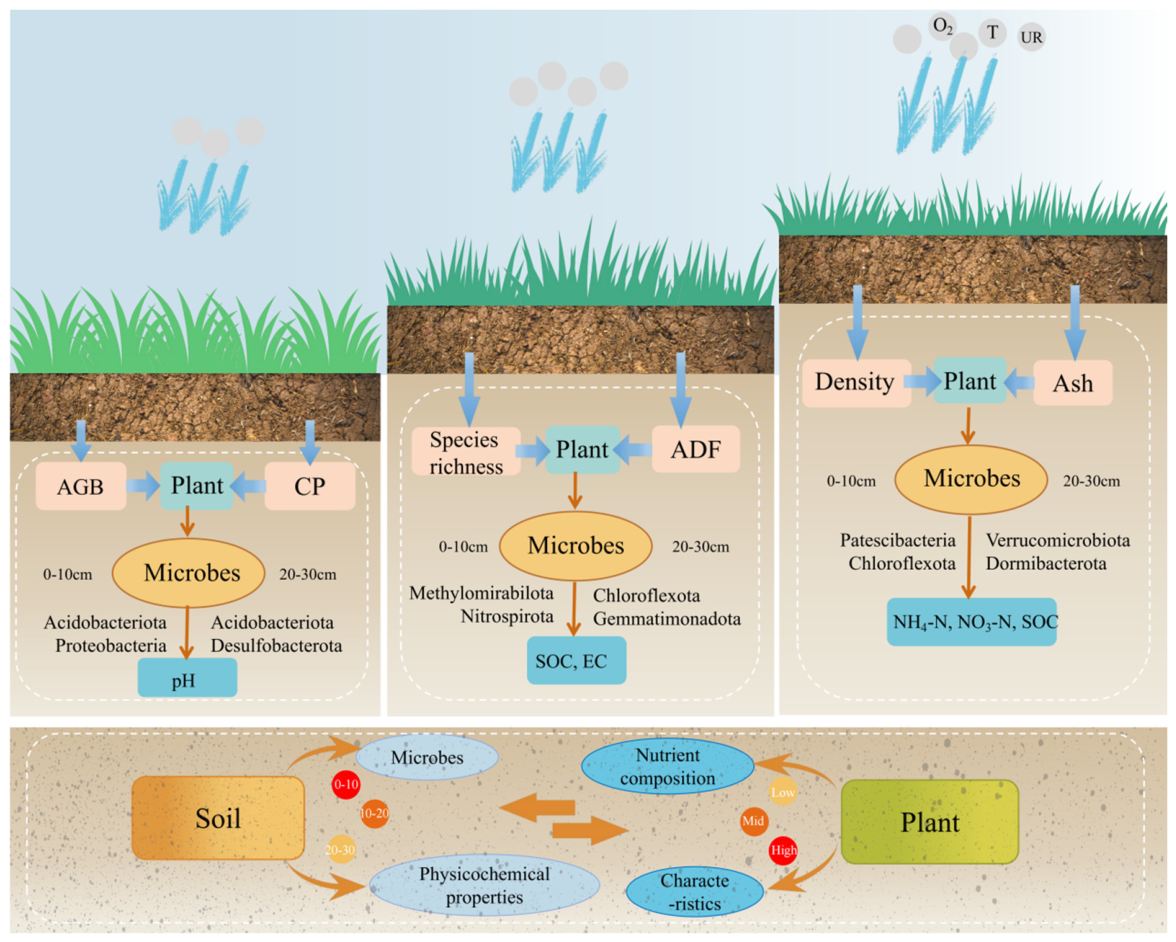
Altitude and soil depth are interdependent, and they jointly shape the characteristics of plateau ecosystems. As shown in Figure 5, the difference in vegetation characteristics influences the difference in soil physicochemical properties, which further reacts to the microbial community structure, and then forms the feedback mechanism of plant–soil interaction. The yield and quality of the pastures are constrained by vegetation types and environmental conditions, affecting their production and utilization efficiency [29]. This study found that the total AGB significantly decreased with increasing altitude, consistent with observations in the Xizang grassland [30] and the China Sanjiangyuan alpine meadow [10]. The meadow, adapted to high-altitude climates, is covered by low-growing herbaceous and cushion vegetation, leading to reduced biomass [31]. Additionally, linear fitting analysis also indicates that AGB and CWH significantly decrease with increasing altitude. This is because temperature decreases with increasing altitude, which strongly restricts plant growth and nitrogen uptake, thus resulting in higher AGB and CWH at low-altitude than at mid- to high-altitudes areas [24]. The significant decrease in crude protein content at high altitude suggests that the quality of pasture decreased with increasing altitude. Plant nutrient accumulation is associated with plant traits and soil physicochemical environment, and adequate soil nutrients are critical for enhancing forage productivity and quality [1,10].
Figure 5.
The mutual influence between soil and vegetation at different altitudes of alpine ecosystems on the Qinghai–Tibet Plateau, Gannan Tibetan Autonomous Prefecture, Gansu province, China. The length of the arrow represents the degree of influence of climate factors at different altitudes, while the circle represents climate factors. Only some climate factors are labeled. O2, oxygen; T, temperature; UR, ultraviolet radiation; AGB, aboveground biomass; CP, crude protein; ADF, acid detergent fiber; SOC, soil organic carbon; EC, electrical conductivity.
Soil pH serves as a key link between plant growth, microbial activity, and nutrient availability. It not only modulates the morphology of chemical species and nutrient availability but also influences microbial growth and function [4]. In the current study, we confirmed that the soil pH continuously decreases with increasing altitude, which is consistent with the previous studies in mountain ecosystems [32]. This may be due to the fact that at higher altitudes, the environmental condition is relatively colder and wetter, alkaline cations in the soil are more easily leached out, and organic acids accumulate, which leads to soil acidification [33]. Meanwhile, the higher SOC content in mid -to high-altitude regions reflects a significant decrease in microbial decomposition rates under low temperature conditions, allowing SOC to gradually accumulate [34]. Furthermore, the depth-dependent patterns exhibited by NH4+-N and NO3−-N indicate that microbial-mediated nitrogen mineralization and nitrification processes undergo significant adjustments based on changes in environmental conditions and soil depth. This response is likely driven by soil pH and SOC content, which influence microbial activity and thus regulate nitrogen transformation rates [35]. From the perspective of soil layer influence, there are significant differences in physicochemical properties among soils of varying depths. Shallow soils typically exhibit higher organic matter input and more active microbial activity [30]. The forms of inorganic nitrogen present in the soil and its EC can reflect depth-specific microbial and geochemical processes, which are regulated by environmental gradients related to altitude [36].
4.2. Vertical Zonal Response of Soil Bacterial Diversity and Functional Communities to Altitude Gradients on the QTP
The microbial community structure differed markedly between the surface and subsurface soil layers, which is consistent with the previous findings that soil depth strongly influences microbial communities [37]. Similar to observations in the southern Loess Plateau, where abundant taxa show pronounced depth-dependent shifts in diversity and composition [38], we observed partial separation of microbial communities between surface and subsurface soil layers. These patterns indicate vertical differentiation in community composition across soil layers [6]. Across all the altitudes, Proteobacteria were dominant phyla but declined with increasing depth. Their ability to utilize readily decomposable substrates likely explains their surface enrichment [39]. In contrast, oligotrophic microorganisms like Chloroflexota and Dormibacterota adapted to resource-poor environments that increased with soil depth [40]. When comparing microbial patterns at the same soil depth across altitudinal gradients, high-altitude surface soil (0–10 cm) exhibited enrichment of Chloroflexota and Dormibacterota, which were relatively more abundant at high altitude. In the 10–20 cm layer, Methylomirabilota and Dormibacterota were more abundant at mid- and high altitudes, while Verrucomicrobiota dominated in the deeper soils (20–30 cm) at high altitude. These patterns are consistent with the reports that rising temperature reduces the abundance of several cold-adapted bacterial groups, particularly Chloroflexota, Dormibacterota, and Desulfobacterota [41,42]. Thus, the observed altitudinal patterns may be associated with climatic differences reported across altitudes.
Predicted functional potentials also varied across altitude and soil depth. In the low-altitude surface soils (L1), a suite of carbon- and nitrogen-related pathways, including ureolysis, nitrogen fixation, fermentation, chitin degradation, aromatic compound degradation, and aerobic heterotrophy, were significantly enriched, reflecting high organic matter inputs and active microbial turnover [43,44]. Similar enrichment occurred in mid-altitude surface soils (M1). In contrast, the deepest high-altitude soil group (H3) was associated with higher predicted relative abundances of functional groups related to nitrification and aerobic ammonia oxidation, suggesting an increased contribution of taxa potentially associated with chemolithotrophic metabolism. This functional profile aligns with the increased relative abundance of Nitrospirota (e.g., Nitrospirota_A_437815), a lineage containing canonical and complete ammonia oxidizers [45,46,47]. Together, these results suggest that carbon-dominated microbial metabolisms prevail in nutrient-rich surface soils, whereas nitrogen transformation pathways become increasingly important in deeper and high-altitude soils.
4.3. Associations Among Soil Properties, Vegetation Characteristics, and Microbial Communities
Along the altitudinal gradient, soil pH and nitrogen variables showed significant associations with microbial community composition in the RDA analyses. These observations are consistent with previous studies reporting associations between soil pH and bacterial community patterns in alpine grasslands [5]. Increasing altitude is typically associated with reduced temperature and plant biomass, which likely constrain SOC inputs while modifying nitrogen cycling processes, thereby strengthening the associations between pH and NH4+-N on microbial assemblages [48,49]. Accordingly, pH and NH4+-N remained significantly associated with the dominant bacterial taxa, including Actinobacteriota, Verrucomicrobiota, and Proteobacteria, particularly at high altitude [50]. Vegetation effects on microbial α-diversity also varied with altitude, with low-altitude diversity closely linked to vegetation quality indicators, suggesting an indirect a potential indirect association through soil nutrient conditions [51].
Associations between microbial communities and vegetation characteristics also varied across soil layers. Surface soils may receive greater inputs of plant residues and root-derived materials than deeper layer. In the surface soil (0–10 cm), plentiful inputs of organic matter from plant litter and root exudates favor fast-growing, copiotrophic taxa, such as Proteobacteria and Actinobacteria [52]. With increasing depth, declining labile carbon and a greater reliance on inorganic nitrogen likely favor oligotrophic and chemolithotrophic taxa that are adapted to low-carbon conditions, including Verrucomicrobiota and ammonia-oxidizing archaea; this is consistent with the patterns reported in previous studies [6,53]. At the 0–10 cm layer, microbial α-diversity showed a significant Mantel association with community-weighted height (CWH). However, labile carbon availability, oxygen conditions, and microbial functional activities were not directly measured in this study.
ASV-level co-occurrence network properties varied across soil depths and altitude zones. Specifically, the number of network edges sharply decreased from the surface to deep soil across low-, mid-, and high-altitude sites, consistent with previous findings that soil depth affects microbial interactions by changing resource availability and environmental conditions [54]. Research on peatlands shows that as soil depth increases, the positive interaction ratio and clustering coefficient rise while negative interactions decline, indicating that surface and deeper soils have distinct topological structures, with generally fewer coexisting connections in deeper soils [55]. Network topology also varied across altitude zones. High-altitude networks showed lower connectivity and higher modularity than the corresponding low- and mid-altitude networks, suggesting a more compartmentalized co-occurrence structure [56]. The proportions of positive and negative co-occurrence associations also differed among altitude zones and soil layers. These observations are broadly consistent with previous studies reporting altitudinal variation in microbial network topology and complexity [57]. However, the present correlation-based networks describe statistical co-occurrence patterns and do not demonstrate direct ecological interactions, such as cooperation, competition, or symbiosis. In addition, temperature, humidity, and resource availability were not included as explanatory variables in the network analyses; therefore, their potential contributions to the observed network patterns cannot be directly evaluated. Therefore, these co-occurrence patterns should be interpreted as statistical correlations that provide clues for potential ecological mechanisms.
5. Conclusions
Vegetation characteristics, soil physicochemical properties, bacterial community composition, predicted functional potentials, and ASV-level co-occurrence network properties varied across altitude zones and soil depths in the sampled alpine grasslands. AGB and CWH were negatively associated with altitude. On the surface soil layer, carbon-driven communities, with complex coexistence networks, are dominant, whereas the deeper layers exhibit simplified networks that are dominated by nutrient-poor and nitrogen cycling taxa. High-altitude networks showed lower connectivity and higher modularity than low- and mid-altitude networks, whereas depth-related network variation differed among altitudes. Together, these observations suggest links among vegetation, soil conditions, and bacterial community patterns but do not establish causal pathways or direct microbial interactions. Seasonal monitoring, manipulative experiments, and direct functional measurements are needed to evaluate the proposed mechanisms.
Supplementary Materials
The following supporting information can be downloaded at https://www.mdpi.com/article/10.3390/biology15181663/s1, Table S1. The effects of altitude and soil depth on soil physicochemical properties; Table S2. Effects of altitudes and soil depths on α-diversity of microbial community of soil collected from Gannan Alpine Meadow; Table S3. Summary of redundancy analysis (RDA) model statistics for different altitudes and soil depths; Table S4. Topological properties of bacterial co-occurrence networks across three altitude zones and three soil depths; Figure S1. Linear regression analysis between vegetation characteristics and altitude gradient. (A) aboveground biomass; (B) species richness; (C) community weighted height; (D) density; Figure S2. Venn diagram displaying shared and individual bacterial ASVs in different soil depths at low, middle and high altitude. L1, L2, L3, M1, M2, M3, H1, H2, and H3 represent soil depths of 0–10, 10–20 and 20–30 cm at low, middle and high altitude, respectively; the same applies to the figures below; Figure S3. Principal component analysis (PCA) at different soil depths and altitudes. (A, B and C) represent PCA plots among different soil depths of low, middle and high altitude, respectively; (D, E and F) represent PCA plots at the same soil depth but different altitudes; Figure S4. Differential microbes at genus levels along soil depths (A) and altitudinal gradients (B). L1, L2, L3, M1, M2, M3, H1, H2, and H3 represent soil depths of 0–10, 10–20 and 20–30 cm at low, middle and high altitude, respectively. Different lowercase letters represent significant differences with p < 0.05.
Author Contributions
Conceptualization, X.G., Z.P., F.H. and T.R.; methodology, X.G. and X.W.; investigation, X.G., X.Y., X.W., R.C., S.Y. and T.R.; resources, F.H., Z.P. and T.R.; data curation, X.G.; writing—original draft preparation, X.G.; writing—review and editing, T.R., Z.P. and P.Y.; supervision, F.H., P.Y. and T.R.; funding acquisition, T.R. All authors have read and agreed to the published version of the manuscript.
Funding
This research was funded by the National Key Research and Development Program of China (2021YFD1300504; 2025YFE0212000), Key Research and Development Program of Gannan Tibetan Autonomous Prefecture (2025ZY1N005), Gansu Province Innovation Platform Plan Project (26JDWA001) and High-End Foreign Experts Recruitment Plan (H20240491).
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
The data presented in this study are openly available in NCBI Sequence Read Archive (SRA) at https://www.ncbi.nlm.nih.gov/bioproject/PRJNA1208410 (accessed on 5 January 2025), reference number PRJNA1208410.
Acknowledgments
We greatly appreciate that Shree Pandy from the College of Pastoral Agriculture Science and Technology, Lanzhou University, critically reviewed and edited the manuscript.
Conflicts of Interest
The authors declare no conflicts of interest.
References
- Philippot, L.; Chenu, C.; Kappler, A.; Rillig, M.C.; Fierer, N. The interplay between microbial communities and soil properties. Nat. Rev. Microbiol. 2023, 22, 226–239. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Falkowski, P.G.; Fenchel, T.; Delong, E.F. The microbial engines that drive earth’s biogeochemical cycles. Science 2008, 320, 1034–1039. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Körner, C. The use of ‘altitude’ in ecological research. Trends Ecol. Evol. 2007, 22, 569–574. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Rousk, J.; Bååth, E.; Brookes, P.C.; Lauber, C.L.; Lozupone, C.; Caporaso, J.G.; Knight, R.; Fierer, N. Soil bacterial and fungal communities across a pH gradient in an arable soil. ISME J. 2010, 4, 1340–1351. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, B.; Jiao, S.; Luo, S.; Ma, B.; Qi, W.; Cao, C.; Zhao, Z.; Du, G.; Ma, X. High soil pH enhances the network interactions among bacterial and archaeal microbiota in alpine grasslands of the Tibetan Plateau. Environ. Microbiol. 2021, 23, 464–477. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Eilers, K.G.; Debenport, S.; Anderson, S.; Fierer, N. Digging deeper to find unique microbial communities: The strong effect of depth on the structure of bacterial and archaeal communities in soil. Soil Biol. Biochem. 2012, 50, 58–65. [Google Scholar] [CrossRef] [Scilit]
- Ji, L.; Shen, F.; Liu, Y.; Yang, Y.; Wang, J.; Purahong, W.; Yang, L. Contrasting altitudinal patterns and co-occurrence networks of soil bacterial and fungal communities along soil depths in the cold-temperate montane forests of China. CATENA 2022, 209, 105844. [Google Scholar] [CrossRef] [Scilit]
- Xu, Z.; Wang, Y.; Sun, D.; Li, H.; Dong, Y.; Wang, Z.; Wang, S. Soil nutrients and nutrient ratios influence the ratios of soil microbial biomass and metabolic nutrient limitations in mountain peatlands. CATENA 2022, 218, 106528. [Google Scholar] [CrossRef] [Scilit]
- Wang, Z.; Yang, G.; Yi, S.; Chen, S.; Wu, Z.; Guan, J.; Zhao, C.; Zhao, Q.; Ye, B. Effects of environmental factors on the distribution of plant communities in a semi-arid region of the Qinghai-Tibet Plateau. Ecol. Res. 2012, 27, 667–675. [Google Scholar] [CrossRef] [Scilit]
- Chen, D.; Li, Q.; Liu, Z.; He, F.Q.; Chen, X.; Xu, S.X.; Zhao, X.Q.; Zhao, L. Variations of forage yield and nutrients with altitude gradients and their influencing factors in slpine meadow of Sanjiangyuan, China. J. Soil Sci. Plant Nutr. 2020, 20, 2164–2174. [Google Scholar] [CrossRef] [Scilit]
- Dlamini, P.; Sekhohola Dlamini, L.M.; Cowan, A.K. Soil-microbial interactions. Front. Microbiol. 2023, 14, 1213834. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, R.; Tian, X.; Xiang, Q.; Penttinen, P.; Gu, Y. Response of soil microbial community structure and function to different altitudes in arid valley in Panzhihua, China. BMC Microbiol. 2022, 22, 86. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yu, J.; Li, S.; Sun, X.; Zhou, W.; He, L.; Zhao, G.; Chen, Z.; Bai, X.; Zhang, J. The impact and determinants of mountainous topographical factors on soil microbial community characteristics. Microorganisms 2023, 11, 2878. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- AOAC International. Official Methods of Analysis, 18th ed.; AOAC International: Gaithersburg, MD, USA, 2005. [Google Scholar]
- Li, H.; Li, J.; He, Y.L.; Li, S.J.; Liang, Z.S.; Peng, C.H.; Polle, A.; Luo, Z.B. Changes in carbon, nutrients and stoichiometric relations under different soil depths, plant tissues and ages in black locust plantations. Acta Physiol. Plant. 2013, 35, 2951–2964. [Google Scholar] [CrossRef] [Scilit]
- Ren, C.; Zhang, W.; Zhong, Z.; Han, X.; Yang, G.; Feng, Y.; Ren, G. Differential responses of soil microbial biomass, diversity, and compositions to altitudinal gradients depend on plant and soil characteristics. Sci. Total Environ. 2018, 610, 750–758. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fatima, F.; Pathak, N.; Rastogi Verma, S. An improved method for soil DNA extraction to study the microbial assortment within rhizospheric region. Mol. Biol. Int. 2014, 2014, 518960. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, Q.; Wang, P.; Zou, C.; Ge, F.; Li, F.; Liu, Y.; Zhang, D.; Tian, J. Dynamics of dominant rhizospheric microbial communities responsible for trichlorfon absorption and translocation in maize seedlings. J. Hazard. Mater. 2023, 451, 131096. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bolyen, E.; Rideout, J.R.; Dillon, M.R.; Bokulich, N.A.; Abnet, C.C.; Al-Ghalith, G.A.; Alexander, H.; Alm, E.J.; Arumugam, M.; Asnicar, F.; et al. Reproducible, interactive, scalable and extensible microbiome data science using QIIME 2. Nat. Biotechnol. 2019, 37, 852–857, Correction in Nat. Biotechnol. 2019, 37, 1091. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Callahan, B.J.; McMurdie, P.J.; Rosen, M.J.; Han, A.W.; Johnson, A.J.A.; Holmes, S.P. DADA2: High-resolution sample inference from Illumina amplicon data. Nat. Methods 2016, 13, 581–583. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bokulich, N.A.; Kaehler, B.D.; Rideout, J.R.; Dillon, M.; Bolyen, E.; Knight, R.; Huttley, G.A.; Caporaso, J.G. Optimizing taxonomic classification of marker-gene amplicon sequences with QIIME 2’s q2-feature-classifier plugin. Microbiome 2018, 6, 90. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Quast, C.; Pruesse, E.; Yilmaz, P.; Gerken, J.; Schweer, T.; Yarza, P.; Peplies, J.; Glöckner, F.O. The SILVA ribosomal RNA gene database project: Improved data processing and web-based tools. Nucleic Acids Res. 2013, 41, D590–D596. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dixon, P. Vegan, a package of R functions for community ecology. J. Veg. Sci. 2003, 14, 927–930. [Google Scholar] [CrossRef]
- Yoshiki, V.; Pirrung, M.; Gonzalez, A.; Knight, R. Emperor: A tool for visualizing high-throughput microbial community data. GigaScience 2013, 2, 16. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Louca, S.; Parfrey, L.W.; Doebeli, M. Decoupling function and taxonomy in the global ocean microbiome. Science 2016, 353, 1272–1277. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Barberán, A.; Bates, S.; Casamayor, E.; Fierer, N. Using network analysis to explore co-occurrence patterns in soil microbial communities. ISME J. 2012, 6, 343–351, Correction in ISME J. 2014, 8, 952. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Quan, Q.; He, N.; Zhang, R.; Wang, J.; Luo, Y.; Ma, F.; Pan, J.; Wang, R.; Liu, C.; Zhang, J.; et al. Plant height as an indicator for alpine carbon sequestration and ecosystem response to warming. Nat. Plants 2024, 10, 890–900. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sun, L.; Sun, J.; Wu, J.; Du, Z.; Chen, Y.; Wang, Y.; Liu, M.; Chen, W.; Liang, E. Plant community traits and functions mediate the biomass trade-off of alpine grasslands along precipitation gradients on the Tibetan Plateau. J. Plant Ecol. 2023, 16, rtad009. [Google Scholar] [CrossRef] [Scilit]
- Shi, Y.; Ma, Y.; Ma, W.; Liang, C.; Zhao, X.; Fan, J.; He, J. Large scale patterns of forage yield and quality across Chinese grasslands. Chin. Sci. Bull. 2012, 58, 1187–1199. [Google Scholar] [CrossRef] [Scilit]
- Bhandari, J.; Zhang, Y.J. Effect of altitude and soil properties on biomass and plant richness in the grasslands of Tibet, China, and Manang District, Nepal. Ecosphere 2019, 10, e02915. [Google Scholar] [CrossRef] [Scilit]
- Pérez, C.A.; Frangi, J.L. Grassland biomass dynamics along an altitudinal gradient in the Pampa. J. Range Manag. 2000, 53, 518–528. [Google Scholar] [CrossRef] [Scilit]
- Shamsher, A.; Hussain, I.; Hussain, S.; Hussain, A.; Ali, H.; Ali, M. Effect of Altitude on Forest Soil Properties at Northern Karakoram. Eurasian Soil Sci. 2019, 52, 1159–1169. [Google Scholar] [CrossRef] [Scilit]
- Wang, B.; Li, H.; Li, X.; Liang, X.; Wang, L.; Zhan, F.; He, Y.; Si, Z.; He, S. Response of Soil Organic Carbon Components in Pinus yunnanensis Stand to Altitude Variation. Agronomy 2026, 16, 4. [Google Scholar] [CrossRef] [Scilit]
- Liu, Q.; Zhang, A.; Li, X.; Yin, J.; Zhang, Y.; Sun, O.; Jiang, Y. Changes in soil organic and inorganic carbon with elevation in a dry alpine rangeland of the northern Qinghai Tibet Plateau. Biogeosciences 2025, 22, 4123–4133. [Google Scholar] [CrossRef] [Scilit]
- Cheng, Y.; Wang, J.; Mary, B.; Zhang, J.; Cai, Z.; Chang, S. Soil pH has contrasting effects on gross and net nitrogen mineralizations in adjacent forest and grassland soils in central Alberta, Canada. Soil Biol. Biochem. 2013, 57, 848–857. [Google Scholar] [CrossRef] [Scilit]
- Husson, O. Redox potential (Eh) and pH as drivers of soil/plant/microorganism systems: A transdisciplinary overview pointing to integrative opportunities for agronomy. Plant Soil 2012, 362, 389–417. [Google Scholar] [CrossRef] [Scilit]
- Chu, H.; Sun, H.; Tripathi, B.; Adams, J.; Huang, R.; Zhang, Y.; Shi, Y. Bacterial community dissimilarity between the surface and subsurface soils equals horizontal differences over several kilometers in the western Tibetan Plateau. Environ. Microbiol. 2016, 18, 1523–1533. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Peng, Z.; Wang, Z.; Liu, Y.; Yang, T.; Chen, W.; Wei, G.; Jiao, S. Soil phosphorus determines the distinct assembly strategies for abundant and rare bacterial communities during successional reforestation. Soil Ecol. Lett. 2021, 3, 342–355. [Google Scholar] [CrossRef] [Scilit]
- Jiao, N.; Luo, T.; Chen, Q.; Zhao, Z.; Xiao, X.; Liu, J.; Jian, Z.; Xie, S.; Thomas, H.; Herndl, G.J.; et al. The microbial carbon pump and climate change. Nat. Rev. Microbiol. 2024, 22, 408–419. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, J.; Peng, Z.; Tu, H.; Qiu, Y.; Liu, Y.; Li, X.; Gao, H.; Pan, H.; Chen, B.; Liang, C.; et al. Oligotrophic microbes are recruited to resist multiple global change factors in agricultural subsoils. Environ. Int. 2024, 183, 108429. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lin, D.; Du, S.; Zhao, Z.; Zhang, T.; Wang, L.; Zhang, Q.; Zhou, S.Y.D.; Graham, D.W.; Tissue, D.T.; Zhu, D.; et al. Climate warming fuels the global antibiotic resistome by altering soil bacterial traits. Nat. Ecol. Evol. 2025, 9, 1512–1526. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Guo, X.; Yuan, M.; Lei, J.; Shi, Z.; Zhou, X.; Li, J.; Deng, Y.; Yang, Y.; Wu, L.; Luo, Y.; et al. Climate warming restructures seasonal dynamics of grassland soil microbial communities. mLife 2022, 15, 245–256. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fierer, N.; Bradford, M.A.; Jackson, R.B. Toward an ecological classification of soil bacteria. Ecology 2007, 88, 1354–1364. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Han, S.; Luo, X.; Hao, X.; Ouyang, Y.; Zeng, L.; Wang, L.; Wen, S.; Wang, B.; Van Nostrand, J.D.; Chen, W.; et al. Microscale heterogeneity of the soil nitrogen cycling microbial functional structure and potential metabolism. Environ. Microbiol. 2021, 23, 1199–1209. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bahram, M.; Espenberg, M.; Pärn, J.; Lehtovirta-Morley, L.; Anslan, S.; Kasak, K.; Kõljalg, U.; Liira, J.; Maddison, M.; Moora, M.; et al. Structure and function of the soil microbiome underlying N2O emissions from global wetlands. Nat. Commun. 2022, 13, 1430. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hamonts, K.; Clough, T.J.; Stewart, A.; Clinton, P.W.; Richardson, A.E.; Wakelin, S.A.; O’Callaghan, M.; Condron, L.M. Effect of nitrogen and waterlogging on denitrifier gene abundance, community structure and activity in the rhizosphere of wheat. FEMS Microbiol. Ecol. 2013, 83, 568–584. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sun, S.; Lu, C.; Liu, J.; Williams, M.A.; Yang, Z.; Gao, Y.; Hu, X. Antibiotic resistance gene abundance and bacterial community structure in soils altered by ammonium and nitrate concentrations. Soil Biol. Biochem. 2020, 149, 107965. [Google Scholar] [CrossRef] [Scilit]
- Wang, J.; Cao, P.; Hu, H.; Li, L.; Han, L.; Zhang, L.; Zheng, Y.; Hu, J. Altitudinal distribution patterns of soil bacterial and archaeal communities along Mt. Shegyla on the Tibetan Plateau. Microbial. Ecol. 2015, 69, 135–145. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yang, Y.; Gao, Y.; Wang, S.; Xu, D.; Yu, H.; Wu, L.; Lin, Q.; Hu, Y.; Li, X.; He, Z.; et al. The microbial gene diversity along an elevation gradient of the Tibetan grassland. ISME J. 2014, 8, 430–440. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xiang, J.; Gu, J.; Wang, G.; Bol, R.; Yao, L.; Fang, Y.; Zhang, H. Soil pH controls the structure and diversity of bacterial communities along elevational gradients on Huangshan, China. Eur. J. Soil Biol. 2024, 120, 103586. [Google Scholar] [CrossRef] [Scilit]
- Liu, L.; Zhu, K.; Wurzburger, N.; Zhang, J. Relationships between plant diversity and soil microbial diversity vary across taxonomic groups and spatial scales. Ecosphere 2020, 11, e02999. [Google Scholar] [CrossRef] [Scilit]
- Liao, J.; Dou, Y.; Yang, X.; An, S. Soil microbial community and their functional genes during grassland restoration. J. Environ. Manag. 2023, 325, 116488. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lu, X.; Seuradge, B.J.; Neufeld, J.D. Biogeography of soil Thaumarchaeota in relation to soil depth and land usage. FEMS Microbiol. Ecol. 2017, 93, fiw246. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mundra, S.; Kjønaas, O.J.; Morgado, L.N.; Krabberød, A.K.; Ransedokken, Y.; Kauserud, H. Soil depth matters: Shift in composition and inter-kingdom co-occurrence patterns of microorganisms in forest soils. FEMS Microbiol. Ecol. 2021, 97, fiab022. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhao, M.; Wang, M.; Zhao, Y.; Hu, N.; Qin, L.; Ren, Z.; Wang, G.; Jiang, M. Soil microbial abundance was more affected by soil depth than the altitude in peatlands. Front. Microbiol. 2022, 13, 1068540. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, Z.; Xu, Y.; Wang, X.; Ma, T.; Liu, Y.; Qin, X.; Zhang, W.; Chen, T.; Liu, G.; Zhang, B. Altitudinal patterns of bacterial communities across soil layers in the alpine meadows of the Qinghai-Tibet Plateau. Ecol. Indic. 2025, 171, 113185. [Google Scholar] [CrossRef] [Scilit]
- Chen, W.; Wang, J.; Chen, X.; Meng, Z.; Xu, R.; Duo, D.; Zhang, J.; He, J.; Wang, Z.; Chen, J.; et al. Soil microbial network complexity predicts ecosystem function along elevation gradients on the Tibetan Plateau. Soil Biol. Biochem. 2022, 172, 108766. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.