


Abstract
Soybean [Glycine max (L.) Merrill] is an important crop in southern Africa where it is cultivated in a wide range of agro-ecologies. Both spatial and seasonal variability is high in the region. As a result, breeders aim to release varieties with a fine balance of high productivity potential and stability. Genotype × environment interaction (GEI) limits the selection of superior genotypes in heterogeneous environments consequently slowing down breeding progress. This study determined the magnitude of GEI effects and genotype superiority index of soybean genotypes of different ages across three countries in southern Africa. Forty-two soybean genotypes that were released between 1966 and 2013 were evaluated for two seasons at thirteen diverse locations across the three countries. Additive main effects and multiplicative interaction (AMMI) and genotype superiority index tools were used to analyse both productivity and stability performance of these genotypes. The AMMI analysis showed that grain yield variation due to genotypes, environments main effects and GEI were highly significant (p < 0.001). Environments explained the greatest proportion (77%) of the total treatment sum of squares followed by GEI (17.4%) and genotypes (5.6%), justifying the need for multi-environmental trials over many seasons in this region. The two methods were useful in discriminating and identifying common productive and stable genotypes of different ages. The top four high-yielding (>5.0 tha−1) genotypes displayed both stability and genotype superiority index. These findings have important implications for soybean genotype recommendations, breeding progress, and strategy.
1. Introduction
Soybean [Glycine max (L.) Merrill] is an important leguminous crop which is used for human food and industrial purposes world-wide [1,2,3]. It is also useful as a supplement in livestock feed and in improving soil fertility through biological nitrogen fixation [4,5,6]. Soybean is important as a cash crop, nutrition and food security crop in many countries including southern Africa. The crop is grown by both the high and low-input farmers in variable environments. Therefore, productive and stable genotypes are desirable in soybean production.
In southern Africa, the exchange and movement of genotypes of field crops such as soybean across national borders was approved recently. In addition, some local plant breeding companies operate from multiple representative branches in more than one country which enables them to market their genotypes widely in the region. Therefore, genotypes with wide ecological amplitudes are advantageous in such situations. However, soybean is cultivated in a wide range of agro-ecologies (environments) with varying edaphic conditions, latitude and management regimes in the region. The crop is exposed to the influence of genotype by environment interaction (GEI) which can potentially affect the productivity and profitability of the crop. In addition, GEI can limit genetic progress [7]. Nonetheless, a significant GEI can be exploited for selecting stable genotypes for specific environments particularly if potential genotypes are evaluated over a range of locations and years to determine superior and stable genotypes [8,9]. It is generally expected that new genotypes would be superior for both yield and stability when grown in the region of their adaptation. This is due to the fact that breeders are expected to derive new genotypes from elite by elite crosses every year which results in incremental yield performance and stability over the years. However, this might be com-promised by the quest to balance mean performance with diversity, especially in public breeding programmes. Therefore, the objectives of this study were to determine (i) the magnitude of GEI effect on soybean grain yield; (ii) the stability and adaptation; and (iii) the genotype superiority index (GSI) (which is equivalent to the cultivar superiority index as indicated below) of elite soybean genotypes of different ages across three soybean growing countries in southern Africa.
2. Materials and Methods
2.1. Genotypes and Test Environments
Forty-two soybean genotypes, which were released in Zimbabwe during the 1966–2013 period, were utilized in the study. For convenience of the study, the genotypes were coded and their respective designated names indicated (Table 1). The genotypes largely consisted of medium maturity types which require about 106–131 days to mature. The field trials were conducted in three southern Africa countries, namely Malawi, Zambia, and Zimbabwe over two cropping seasons (2010/2011 and 2011/2012). Five and eight test locations were used during the 2010/2011 and 2011/2012 cropping seasons, respectively, resulting in a total of 13 environments (season × location combination). The locations represented the major soybean production ecologies in the region (Table 2).
Table 1.
Soybean genotypes evaluated at 13 test environments in southern Africa.
Table 2.
Physical and weather characteristics of the study locations.
The environments were characterized by temperatures that ranged from 13.0 °C to 30.0 °C over the two seasons. The location at the Agricultural Research Trust in Zimbabwe was the coolest while Bvumbwe Research Station in Malawi, was relatively warm. The temperatures were generally favorable for the vegetative growth and development of the crop since stressfully higher temperatures negatively affect pollen viability (and hence grain yield) [10].
2.2. Experimental Design and Management
The experiment was designed as a 6 × 7 rectangular lattice with three replications for each test environment. Planting was carried out between the last week of November up to mid-December across all of the sites and seasons. The experimental unit consisted of six rows, 5.0 m long and spaced at 0.45 m. In each row, seed was planted at 6.3 cm apart resulting in a plant population of approximately 350,000 plants ha−1. Assuming that 10% of the seed did not germinate or was lost due to various factors, then number of established plants (or the harvest plant population) was approximately 315,000 plants ha−1. Standard cultural practices for soybean production that included land or seedbed preparation, hand planting, weeding, herbicide application and crop protection were applied at each test environment. Fertilizer (was applied at a rate of 400 kg ha−1 supplying 28 kg ha−1 of N, 68 kg ha−1 of P2O5 and 40 kg ha−1 of K2O. The seed was inoculated with Bradrhizobium japonicum inoculant. Across all of the trial locations, both pre-emergence and post emergence herbicides were used. Lasso (Alachlor 384 EC) (active ingredient = chloroacetanilide) and Gramoxone (active ingredient = paraquat) were mixed and applied together as pre-emergence herbicides at planting at 5.0 L ha−1 and 3.0 L ha−1, respectively. Basagran (active ingredient = sodium salt of Bentazon) and Bateleur Gold 650 EC (active ingredient = Sulfonanilide (Flumetsulam)) were applied as post emergence herbicides at 3.0 L ha−1 and 1.2 L ha−1, respectively. Both herbicides were applied within six weeks post emergence as per recommendation of the manufacturer to control the weeds early. Hand weeding was carried out just before the canopying stage.
Insect pests, notably the soybean looper (Chrysodeixis includens) that sporadically appeared in the field trials were controlled using Thionex 35 EC (active ingredient = endosulfan) and Karate 2.5% EC (active ingredient = Lambda-cyhalothrin) which were applied at 400 mL and 266 mL in 200 L of water, respectively. The looper is common in the soybean crop. The fungicide Shavit (active ingredients = Folpet and Triadimenol), was also applied on the trials (at a rate of 266 mL per 200 L of water ha−1) as a preventative measure against soybean rust (Phakopsora pachyrhizi) that was prevalent in the region [11,12,13]. The initial spraying was carried out at 50 days after planting followed by two subsequent applications at 20 day intervals, thereafter.
All of the trials were harvested manually. Due to the variation in duration to maturity, the harvesting in each experimental unit was carried out at the 95% pod maturity [14]. Consequently, the harvesting at each test location was carried out sequentially. The grain yield was obtained from a net plot (7.92 m2) consisting of four rows measuring 4.4 m long. The grain yield was adjusted for moisture content (calculated at 11%) which is the standard practice in the region.
2.3. Data Analysis
The data sets of the grain yield were subjected to the analysis of variance (ANOVA) model using the model (Equation (1)) and the additive main-effects and multiplicative interaction (AMMI) model [15,16] (Equation (2)) in GenStat 14 software (version, 2011) [17] as follows:
where:
Yger = µ + αg + βe + θge + Ɛger, (ANOVA model)
Yger = μ + αg + βe + N∑n=1 ʎnϛgn ηen + ρge + Ɛger, (AMMI model)
Yger = the grain yield level for genotype g in environment e for replicate r
μ = the grand mean
αg = genotype mean deviations (mean minus the grand mean)
βe = the environment mean deviations
N = the number of singular value decomposition (SVD) axes retained in the model
ʎn = the singular value for SVD axis η
ϛgn = the genotype singular vector values for SVD axis n
θge = the interaction residuals
ρge = the AMMI residuals
Ɛger = the error term and
N∑n=1ʎnϛgn ηen + ρge is equivalent to the interaction term in the ANOVA model.
The computation estimates the level of noise using statistics from the AMMI ANOVA approach and defined noise as the difference between yield estimate and its true mean [15]. Therefore, the percent level of noise in the GE interaction component was estimated as follows:
where:
[100 × (Interaction DF × EMS)]/Interaction Sum of Squares (SS)
Interaction DF = interaction degrees of freedom
EMS = the expected error mean square for the AMMI ANOVA
Interaction SS = interaction sum of squares.
One AMMI biplot was plotted and IPCA1 scores were plotted against genotype and environment means. The stability coefficients displaying genotype superiority index (GSI) were also computed in GenStat 14th Edition [17]. The GSI is similar to the cultivar superiority index [18]. The stability of the genotypes across the environments was estimated by the GSI which is a measure of both productivity and stability hence a favourable tool to identify the desirable genotypes for deployment and use in breeding new genotypes for the region.
3. Results
The analysis of variance showed that soybean grain yield was significantly (p < 0.001) affected by environments main effects, genotypes main effects and genotype by environment interaction (GEI) effects (Table 3). The treatments (genotypes + environments + interactions) accounted for 87.7% of the total grain yield sums of squares using approximately 33.3% of the total degrees of freedom. The genotypes accounted for 4.9% of the total sums of squares and 5.6% of the treatments sums of squares. On the other hand, the environments explained 67.5% of the total sums of squares and 77.0% of the treatments sums of squares. The interactions explained 15.3% of the total sums of squares and 17.4% of the treatments sums of squares. Therefore, the environments accounted for more variation than the interactions (genotype × environment interactions) while the genotypes captured the least variation. The magnitude of the GEI sum of squares was about three-fold larger than that for genotypes implying that there were significant differences in genotypic response to the test environments.
Table 3.
Analysis of variance for full AMMI model for grain yield (kg ha−1) of 42 soybean genotypes evaluated across three countries in southern Africa.
The application of AMMI model for partitioning of GEI showed that the first six multiplicative terms of AMMI were significant (Table 3). However, IPCA1 explained 46.1% of the total interaction sum of squares using about 10.6% of the total interaction degrees of freedom. When IPCA2 was fitted, the two IPCAs explained 58.5% of the total interaction variation using approximately 20.8% of the total interaction degrees of freedom. When the third IPCA was added, the model explained 69.1% of the total interaction using about 30.6% of the total interaction degrees of freedom. The first four IPCAs explained 76.6% of the total interaction variation using approximately 39.9% of the total interaction degrees of freedom. The IPCA5 and IPCA6 were significant and accounted for less than 10% of the sum of squares of the interactions. On the other hand, multiplicative axis from IPCA7 to IPCA9 including the residual captured mostly noise.
The model selection was based on firstly the proportional contribution of each IPCA to genotype × environment interaction and the ratio of noise sum of squares to residual sum of squares. The proportion of noise sum of squares for AMMI3 to its residual sum of squares was almost 1.0 making AMMI3 the most suitable model. In addition, the sum of squares of the first three terms were greater than that of genotypes and highly significant (p < 0.001). Although AMMI3 was the best model, the biplot analysis was generated from IPCA1 since it explained 46.1% of the total interaction sum of squares.
The ranking of the first four AMMI selections per environment for grain yield indicated that the highest (7628 kg ha−1) and lowest (3112 kg ha−1) grain yield per environment was attained at Mapongwe in Zambia (E4) and RARS in Zimbabwe (E1), respectively (Table 4). The results also showed that both old and new genotypes were among the top performers with respect to both yield and stability. The genotype G28, which was released in 2006, was among the top four ranked genotypes in at least seven environments followed by genotype G27, which was released in 1998. In addition, genotype G28, attained >5000 kg ha−1 in at least five environments (Table 5). Nonetheless, only three genotypes (G4, G9 and G33) among the bottom 21 failed to produce ≥5000 kg ha−1 in at least one test environment indicating that there was a strong environmental influence on grain yield. In terms of the GSI, genotype G25 was the most superior followed by genotype G1 while genotype G16 performed the least (Table 5).
Table 4.
Ranking of the first four AMMI selections per environment for grain yield.
Table 5.
AMMI IPCA1 scores and grain yield (kg ha−1) of the top 21 soybean genotypes across 3 countries in southern Africa.
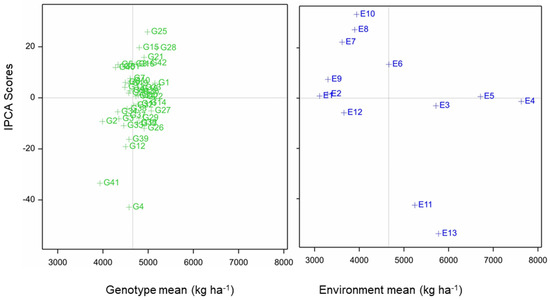
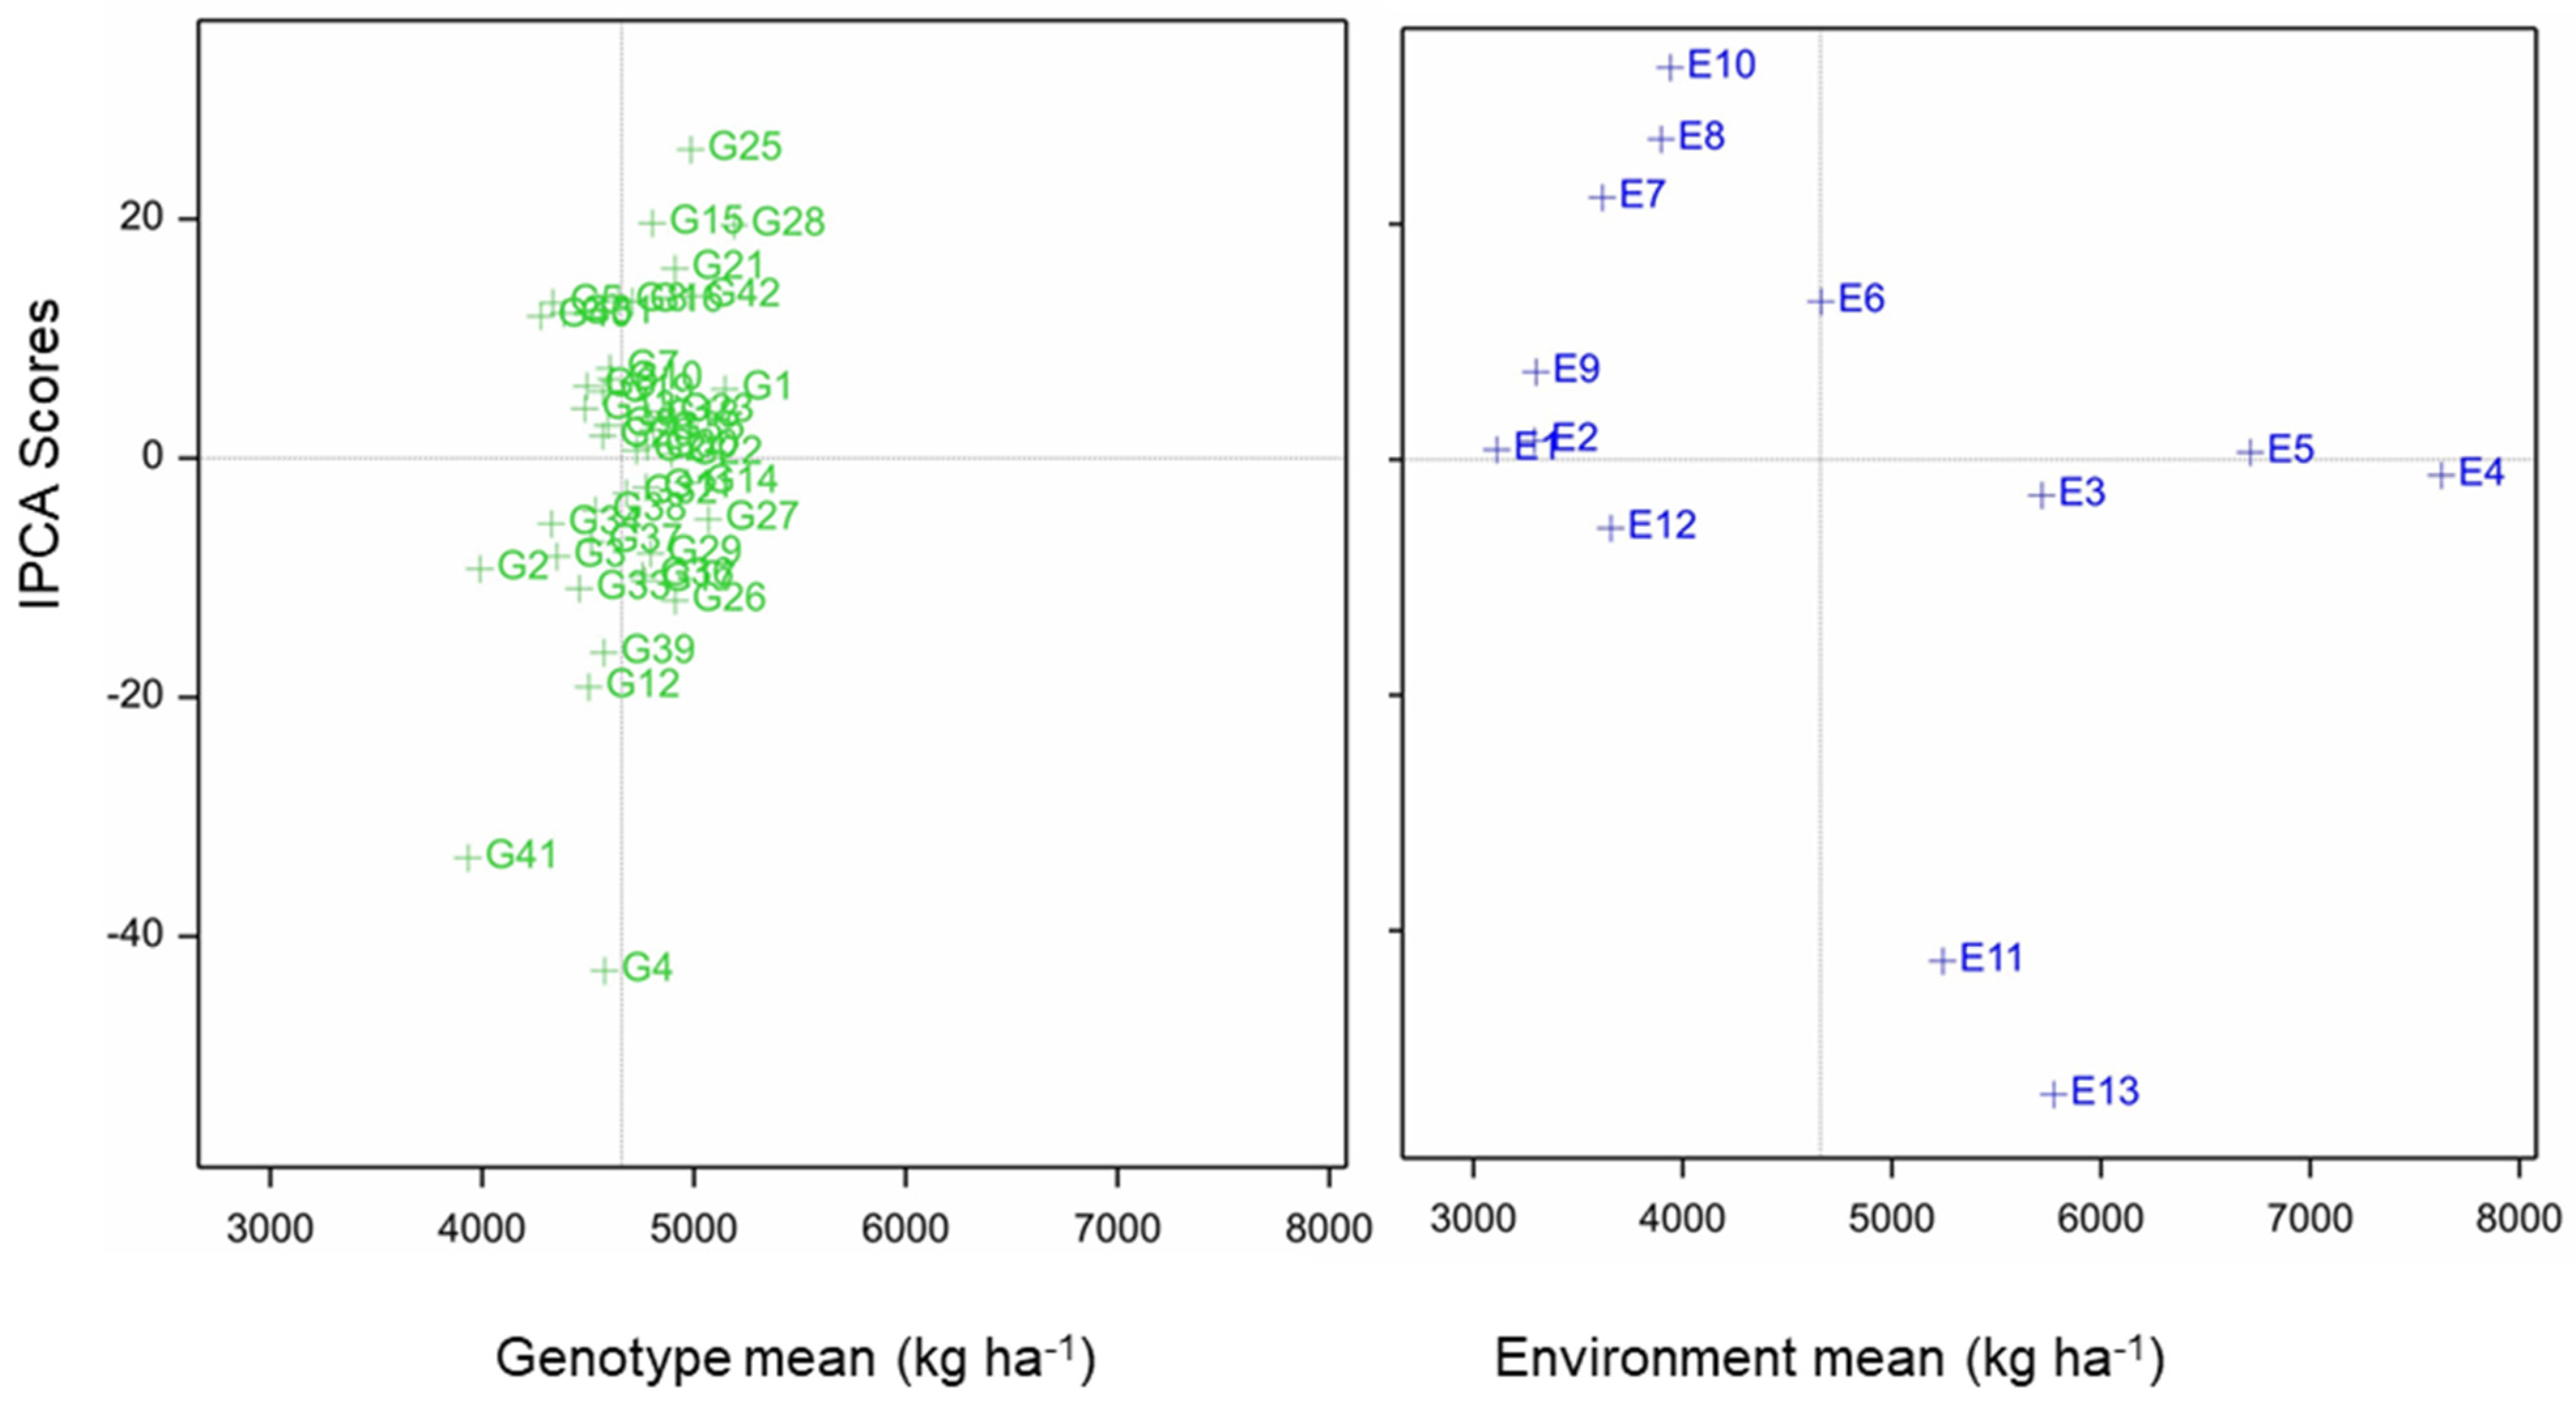
The biplot of the AMMI-1 showed that genotype G25 had the largest positive (>10) interaction with the environments while G4 had the largest negative interaction with environments (Figure 1). Genotype G28 was the overall best performer, combining relative stability and high yield. In addition, genotypes G15, G25, G28, and G42 were relatively stable and produced above average yield but genotype G12 was the most stable since its mean yield was equal to the grand mean. The test environments showed variability in both main effects and interaction. Environments E3, E4, E5, E6, E11, and E13 were classified above the mean grain yield of all of the environments whereas the remainder performed below the average yield (i.e., less than the grand mean yield level). Genotypes and environments with the same sign on the IPCA axis interacted positively whereas those with different signs interacted negatively.
Figure 1.
AMMI-1 biplot of IPCA 1 scores against grain yield for 42 soybean genotypes and 13 environments. E1, Rattray Arnold Research Station, 2010/11; E2, Gwebi Variety Testing Centre, 2010/11; E3, Lusaka West Farm, 2010/11; E4, Mpongwe Development Centre, 2010/11; E5, Bvumbwe Research Station, 2010/11; E6, Rattray Arnold Research Station, 2011/12; E7, Gwebi Variety Testing Centre, 2011/12; E8, Lusaka Farm West, 2011/12; E9, Mpongwe Development Centre, 2011/12; E10, Bvumbwe Research Station, 2011/12; E11, Lilayi Farm, 2011/12; E12, Agricultural Research Trust, 2011/12; E13, Chitedze Research Station, 2011/12; G1 to G42 represent the test genotypes.
4. Discussion
The AMMI analysis of variance for the 42 genotypes that were evaluated across 2 seasons and 13 test environments revealed strong evidence that environment, genotype, and genotype × environment effects were significantly different from each other. Furthermore, the results revealed that the environment component had larger influence on the performance of soybean genotypes, indicating the necessity for testing soybean genotypes at multi-location sites and over years [19]. The huge influence by the environment illustrated its impact on controlling the expression of grain yield. The bottom line was that the environments contributed more to the phenotypic value which has affected the selection efficiency and breeding progress. The presence of GEI complicated the selection process of superior genotypes and reduced the selection efficiency in a soybean breeding program [15]. The magnitude of GEI effect was five times larger than that for the genotypes indicating differences in genotypic responses to test environments. However, although the environment accounted for the highest variation, one could expect the GEI to be higher than what was observed since the environments were sampled from three countries thus, greater variability was expected. Generally, the more variable the environments, the greater the GEI [16]. Nonetheless, the GEI variation (17.4%) was close to the expected, possibly implying that most of the genotypes were widely adapted. This was supported by the clustering pattern of a considerable number of genotypes around the grand mean yield with IPCA values close to zero.
The results of the study also showed a low GEI in respect of the expected proportion of the components of the treatment sum of squares (70:20:10). Therefore, genotypes that combined both high grain yield and stability (G1 and G15) were recommended for cultivation in all areas that were represented by the test locations. In contrast, the genotypes that exhibited high IPCA scores (G2, G4, G5, G7, G16, G17, G18, G31, and G40) were recommended for specific adaptation. The low IPCA values revealed poor interaction with the test environments that were used in the study, thus indicating less responsiveness to environmental changes. However, at least eight genotypes that were grouped in the top third of the mean yield table could be classified as the best genotypes combining both high stability and above average yield performance [20]. On the other hand, genotype G12 which attained the highest stability rating (IPCA score = 0) and combined low GEI and average yield suggested that it was the most suitable for cultivation across sites and seasons. However, its low yield potential makes it unattractive to farmers. The genotypes that showed large interaction with environments were classified as unstable and hence unpredictable in performance but could be recommended for specific adaptation. The differences among the test environments and their clustering patterns could be attributed to differences in latitude, altitude, climatic conditions, duration of the cropping season as well as seasonal effects. Often, the long duration of the cropping season is correlated with high yielding potential [21]. However, lengthy cropping seasons can be prone to meteorological fluctuations as well as the negative effects of soil moisture stress [22,23,24]. For instance, in both chickpea and soybean, pod abortion increased under terminal drought stress [25,26]. Most of the environments produced the least interaction effects suggesting that they were ideal for evaluation and selection since the performance of the genotypes can be stable. In addition, both the IPCA scores and GSI identified genotype G1 and G25 as the highest yielding and most stable. Therefore, the two stability parameters could be used for simultaneously selection for high yield and stability.
The results also showed that the newly released genotypes (which were released during 2005, 2006 and 2012), were generally superior in performance than most of the older genotypes, except G15 which was released in 1989. Therefore, it can be argued that there was sound breeding progress in the region which resulted in a significant build-up of high allele frequency for adaptation, productivity and stability. The performance pattern increased significantly since the genotypes from the earlier decades were generally poorly adapted and unstable as revealed by large IPCA scores and high genotype superiority indices. However, there are surprises of older genotypes outperforming the most recent (2012 and 2013) genotypes. The genotype G28 was found to be relatively best yielding. In addition, the genotype possesses desirable characteristics which include good quality seed, high number of nodes per plant and good standability. It is generally large seeded (average 100 seed weight approximately 25.0 g). Although G25 was released in 2005, it attained high grain yield. However, it is susceptible to soybean rust and frogeye leaf spot (Cercospora sojina) suggesting that it would be costly to produce where these diseases are endemic. Based on our pedigree information, both G1 and G25 were derived from high yielding genetic backgrounds utilizing elite × elite crosses while some of the other subsequent genotypes were derived from elite × exotic or disease resistant crossing combinations.
The outstanding performance of the genotypes G1 and G25 is partly since both were derived from parents with a high yielding background. The parents of both genotypes were selected on the basis of high additive breeding values. The selection of good parents for each new breeding cycle, that have higher additive breeding value than the previous generation is critical and optimizes the genetic gain [27]. This approach enhances rapid increase in the frequency of favourable alleles, which become fixed in the gene pool. Appreciable rates of genetic gain have been observed in many breeding programs through the application of elite × elite crossing strategy [28]. Essentially, this strategy can drive the competitiveness of the soybean breeding program in the region. It is recommended to evaluate the historical data and use it to create and assemble a core set of high performing lines, such as the top four genotypes that were identified in the current study. The inconsistent utilization of the elite × elite crossing strategy partly explains why some older genotypes outperformed some recently released genotypes. Integration of resistance to new diseases, such as soybean rust, without a good background check could have compromised mean performance of new genotypes that were released in the 2010–2013 period.
As a generalization, AMMI analysis showed that 61.9% of the genotypes obtained IPCA values between −10 and 10, possibly indicating average stability across environments. This suggested that stability was accumulated over time through breeding, extensive evaluation and selection. This was affirmed further by the observation that the founder genotype (G2 which was released in 1966) showed poor stability (IPCA score about 30) in comparison with G28 (which was released in 2006 and IPCA value close to zero). Since yield stability is heritable and conditioned by additive gene action, simple selection methods could be applied in breeding programs to advance yield stability and plasticity for cultivation over a wide range of environments [29,30].
This study was different from previous ones in that it considered the implication of soybean genotypic age (i.e., when a genotype was released) for both productivity and stability, both of which can impact on recommendation of genotypes to growers as well as the breeding and selection of new ones in the region. In addition, the conventional breeders in the region have not been using modern stability models (AMMI and GSI) to identify genotypes that combine both high productivity and stability. Instead, they have been using rank analysis based on the simple arithmetic mean to select and advance new genotypes. The application of modern tools will help to improve selection accuracy and identify genotypes that combine both high productivity and stability which is desired in a region with high levels of variability across sites and seasons. In addition, the information generated in this study will be useful to soybean breeders aiming to develop sustainable genotypes adapted to target environments in the region and possibly using the identified genotypes as reference genotypes in the selection process. Moreover, the stable genotypes that were identified in this study provided insights into future studies aimed at identifying the genomic regions that are associated with stability. For instance, a recent study reported that seven genomic regions in six chromosomes of soybean were associated with genotype-by-environment interactions thus opening a novel frontier of genomic assisted breeding aimed at achieving stable performance of soybean [31].
5. Conclusions
The results of this study showed that both new and old genotypes were among the top four which displayed a combination of high yield potential (>5.0 t ha−1), dynamic stability and GSI. These findings have important implications for soybean genotype recommendations, breeding progress and breeding strategy for the region. These results suggested that grain yield in soybean could be maximized through selecting genotypes showing consistently high yield performance across heterogeneous growing environments. The AMMI analysis revealed the relative magnitude and significance of GEI effects and its interaction terms in relation to genotype and environmental effects. The results also showed that GEI was a vital component of soybean yield variation and the biplots provided a good visualization of the response patterns of genotypes and environments. Two genotypes from both the AMMI and GSI analysis were classified under the high yielding category. Overall, the stability measurements demonstrated that >60.0% of the genotypes were, on average, stable across the 13 test environments while the rest were unstable but suitable for specific environments. Considering the two analytical methods (AMMI and GSI), two genotypes (G1 and G25) were among the best and thus could be recommended for cultivation across the three countries and utilization as breeding stocks in programs that aim to improve both stability and productivity of soybean.
Author Contributions
Conceptualization, J.D. and H.M., methodology, P.T., validation, E.T.G., formal analysis, I.M.; investigation, H.M., writing, E.T.G. All authors have read and agreed to the published version of the manuscript.
Funding
This research received no external funding.
Data Availability Statement
Not applicable.
Acknowledgments
The authors would like to acknowledge the support staff who participated in the study at all of the test locations in the three countries.
Conflicts of Interest
The authors declare no conflict of interest.
References
- Qin, P.; Wang, T.; Luo, Y. A review on plant-based proteins from soybean: Health benefits and soy product development. J. Agric. Food Res. 2022, 7, 100265. [Google Scholar] [CrossRef] [Scilit]
- Whaley, R.; Eskandari, M. Genotypic main effect and genotype-by-environment interaction effect on seed protein concentration and yield in food-grade soybeans (Glycine max (L.) Merrill). Euphytica 2019, 215, 33. [Google Scholar] [CrossRef] [Scilit]
- Gwata, E.T.; Nziramasanga, N. Seed protein and oil content in Zimbabwean soyabean (Glycine max L.) varieties. Plant Var. Seeds 2001, 14, 125–128. [Google Scholar]
- Jandong, E.A.; Uguru, M.I.; Oyiga, B.C. Determination of yield stability of seven soybean (Glycine max) genotypes across diverse soil pH levels using GGE biplot analysis. J. Appl. Biosci. 2011, 43, 2924–2941. [Google Scholar]
- Gwata, E.T.; Wofford, D.S.; Boote, K.J.; Blount, A.R.; Pfahler, P.L. Inheritance of promiscuous nodulation in soybean. Crop Sci. 2005, 45, 635–638. [Google Scholar] [CrossRef] [Scilit]
- Mpepereki, S.; Javaheri, F.; Davis, P.; Giller, K.E. Soyabeans and sustainable agriculture: Promiscuous soyabeans in southern Africa. Field Crops Res. 2000, 65, 137–149. [Google Scholar] [CrossRef] [Scilit]
- Mohammadi, R.; Mohammadi, M.; Karimizadeh, R.; Amri, A. Analysis of genotype-by-environment interaction for grain yield of rainfed durum wheat genotypes in warm winter areas of Iran. J. Crop Sci. Biotechnol. 2010, 13, 267–274. [Google Scholar] [CrossRef] [Scilit]
- Abay, F.; Bjørnstad, A. Specific adaptation of barley varieties in different locations in Ethiopia. Euphytica 2000, 167, 181–195. [Google Scholar] [CrossRef] [Scilit]
- Ramburan, S.; Zhou, M.; Labuschagne, M.T. Investigating test site similarity, trait relations and causes of genotype × environment interactions of sugarcane in the Midlands region of South Africa. Field Crops Res. 2012, 129, 71–80. [Google Scholar] [CrossRef] [Scilit]
- Boote, K.J.; Allen, L.H.; Prasad, P.V.V.; Baker, J.T.; Gesch, R.W.; Snyder, A.M.; Pan, D.; Thomas, J.M.G. Elevated temperature and CO2 impacts on pollination, reproductive growth and yield of several globally important crops. J. Agric. Meteorol. 2005, 60, 469–474. [Google Scholar] [CrossRef] [Scilit]
- Jarvie, J.A. A review of soybean rust from a South African perspective. S. Afr. J. Sci. 2009, 105, 103–108. [Google Scholar] [CrossRef] [Scilit]
- McLaren, N.W. Reaction of soybean cultivars to rust caused by Phakopsora pachyrhizi. S. Afr. J. Plant Soil 2008, 25, 49–54. [Google Scholar] [CrossRef] [Scilit]
- Levy, C. Zimbabwe—A country report on soybean rust control. In Proceedings of the VII World Soybean Research Conference; Moscardi, F., Hoffmann-Campo, C.B., Saraiva, O.F., Galerani, P.R., Krzyzanowski, F.C., Carrão-Panizzi, M.C., Eds.; Embrapa: Londrina, Brazil, 29 February 5 March 2004; pp. 340–348. [Google Scholar]
- Nleya, T.; Sexton, P.; Gustafson, K. Soybean growth stages. In iGrow Soybean: Best Management Practices for Soybean Production; Clay, D.E., Carlson, C.G., Clay, S.A., Wagner, L., Deneke, D., Hay, C., Eds.; South Dakota State University, SDSU Extension: Brookings, SD, USA, 2019; pp. 3–34. [Google Scholar]
- Gauch, H.G., Jr. Statistical Analysis of Regional Yield Trials. AMMI Analysis of Factorial Designs; Elsevier: Amsterdam, The Netherlands, 1992; pp. 53–110. [Google Scholar]
- Gauch, H.G.; Zobel, R.W. AMMI analysis of yield trials. In Genotype-by-Environment Interaction; Kang, M.S., Gauch, H.G., Jr., Eds.; CRC Press: Boca Raton, FL, USA, 1996; pp. 85–122. [Google Scholar]
- Payne, R.W.; Murray, D.A.; Harding, S.A.; Baird, D.B.; Soutar, D.M. GenStat for Windows (14th Edition) Introduction; VSN International: Hemel Hempstead, UK, 2011. [Google Scholar]
- Lin, C.S.; Binns, M.R. A superiority measure of cultivar performance for cultivar location data. Can. J. Plant Sci. 1988, 68, 193–198. [Google Scholar] [CrossRef] [Scilit]
- Gurmu, F.; Mohammed, H.; Alemaw, G. Genotype × environment interactions and stability of soybean for grain yield and nutritional quality. Afr. Crop Sci. J. 2009, 17, 87–99. [Google Scholar]
- Fox, P.N.; Cross, J.; Ramagosa, I. Multiple environment testing and genotype × environment interaction. In Statistical Methods for Plant Variety Evaluation; Kempton, R.A., Fox, P.N., Eds.; Chapman and Hall: London, UK, 1997; pp. 742–754. [Google Scholar]
- Miladinovic, J.; Kurosaki, H.; Burton, J.W.; Hrustic, M.; Miladinovic, D. The adaptability of short season soybean genotypes to varying longitudinal regions. Eur. J. Agron. 2006, 25, 243–249. [Google Scholar] [CrossRef] [Scilit]
- Gao, X.-B.; Guo, C.; Li, F.-M.; Li, M.; He, J. High Soybean Yield and drought adaptation being associated with canopy architecture, water uptake, and root traits. Agronomy 2020, 10, 608. [Google Scholar] [CrossRef] [Scilit]
- Basal, O.; Szabo, A. Physiology yield and quality of soybean as affected by drought stress. Asian J. Agric. Biol. 2020, 3, 247–253. [Google Scholar] [CrossRef] [Scilit]
- Teasdale, J.R.; Cavigelli, M.A. Meteorological fluctuations define long-term crop yield patterns in conventional and organic production systems. Sci. Rep. 2017, 7, 688. [Google Scholar] [CrossRef] [Scilit]
- Fang, X.W.; Turner, N.C.; Yan, G.J.; Li, F.M.; Siddique, K.H.M. Flower numbers, pod production, pollen viability, and pistil function are reduced and flower and pod abortion increased in chickpea (Cicer arietinum L.) under terminal drought. J. Exp. Bot. 2010, 61, 335–345. [Google Scholar] [CrossRef] [Scilit]
- Kokubun, M.; Shimada, S.; Takahashi, M. Flower abortion caused by preanthesis water deficit Is not attributed to impairment of pollen in soybean. Crop Sci. 2001, 41, 1517–1521. [Google Scholar] [CrossRef] [Scilit]
- Cobb, J.N.; Juma, R.U.; Biswas, P.S.; Arbelaez, J.D.; Rutkoski, J.; Altin, G.; Hagen, T.; Quinn, M.; Ng, E.H. Enhancing the rate of genetic gain in public-sector plant breeding programs: Lessons from the breeder’s equation. Theor. Appl. Genet. 2019, 132, 627–645. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Farooq, M.U.; Ishaaq, I.; Maqbool, R.A.; Aslam, I.; Taseer, S.; Naqvi, A.; Mustafa, S. Heritability, genetic gain and detection of gene action in hexaploid wheat for yield and its related attributes. AIMS J. 2019, 4, 56–72. [Google Scholar]
- Sajjad, M.; Saif, M.; Murtaza, A.; Bashir, I.; Shahbaz, M.K.; Ali, M.; Sarfarz, M. Gene action study for yield and yield stability related traits in Gossypium hirsutum: An overview. Life Sci. J. 2015, 12, 1–11. [Google Scholar]
- Spehar, C.R. Diallel analysis for grain yield and mineral absorption rate of soybeans grown in acid brazilian savannah soil. Pesq. Agrop. Brasil. 1999, 34, 1003–1009. [Google Scholar] [CrossRef] [Scilit]
- Xavier, A.; Jarquin, D.; Howard, H.; Ramasubramanian, V.; Specht, J.E.; Graef, G.L.; Beavis, W.D.; Diers, B.W.; Song, Q.; Cregan, P.B.; et al. Genome-wide analysis of grain yield stability and environmental interactions in a multiparental soybean population. G3 Genes Genomes Genet. 2018, 8, 519–529. [Google Scholar] [CrossRef] [Scilit] [PubMed]

Publisher’s Note: MDPI stays neutral with regard to jurisdictional claims in published maps and institutional affiliations. |
© 2022 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).