


Abstract
Among gastropods, the ability to swim has developed independently several times, mostly among Heterobranchia. Only a few species of Caenogastropoda are known to have swimming adults. Velutinidae Gray, 1840, is a family of caenogastropods with a fragile shell enclosed by the mantle. The adults of this family are benthic and ectoparasites of ascidians. Here, we present the first recorded instance of a swimming velutinid, Marsenia cf. gemma, filmed in New Caledonia. The swim propulsion method was based on the movement of the snail’s foot, which followed a ∞-shaped curve. This first report changes our perspective on the biology of this family, unexpectedly placing it within the restricted group of swimming caenogastropods.
Text
Swimming is a common behavior among molluscs, and this ability has evolved independently several times during the diversification of this group. Extant species of swimming gastropods mostly belong to Heterobranchia, with a few species in Vetigastropoda and Caenogastropoda. This ability has been achieved using different anatomical structures (e.g., mantle, foot) and propulsion methods (e.g., flapping, undulating, lateral bending, water stroke, jet propulsion) [1]. Among caenogastropods, very few species were observed swimming during adult life, which is mostly benthic, while this behavior is more common during the larval stage, which ensures geographic dispersion and genetic connectivity among populations [2,3].
Velutinidae Gray, 1840, is a family of caenogastropods whose members are distributed worldwide. They are characterized by having the appearance of sea slugs but retaining a fragile and vestigial shell, completely enclosed by the mantle (with a few exceptions) [4]. The velutinid larva is planktotrophic and can remain in the water column for long periods, but the adult is benthic and generally found as an ectoparasite of ascidians [4,5,6]. Here, we report the observation of an actively swimming velutinid, representing not only a first for this family but also one of the few cases among caenogastropods.
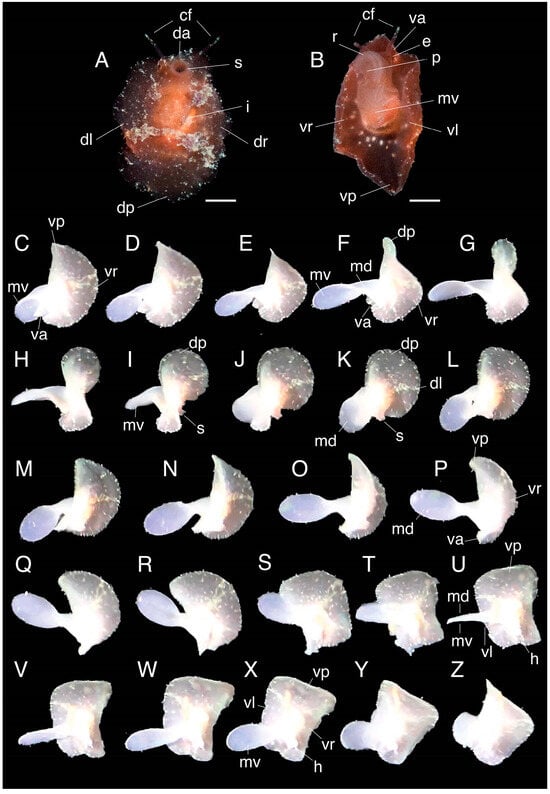
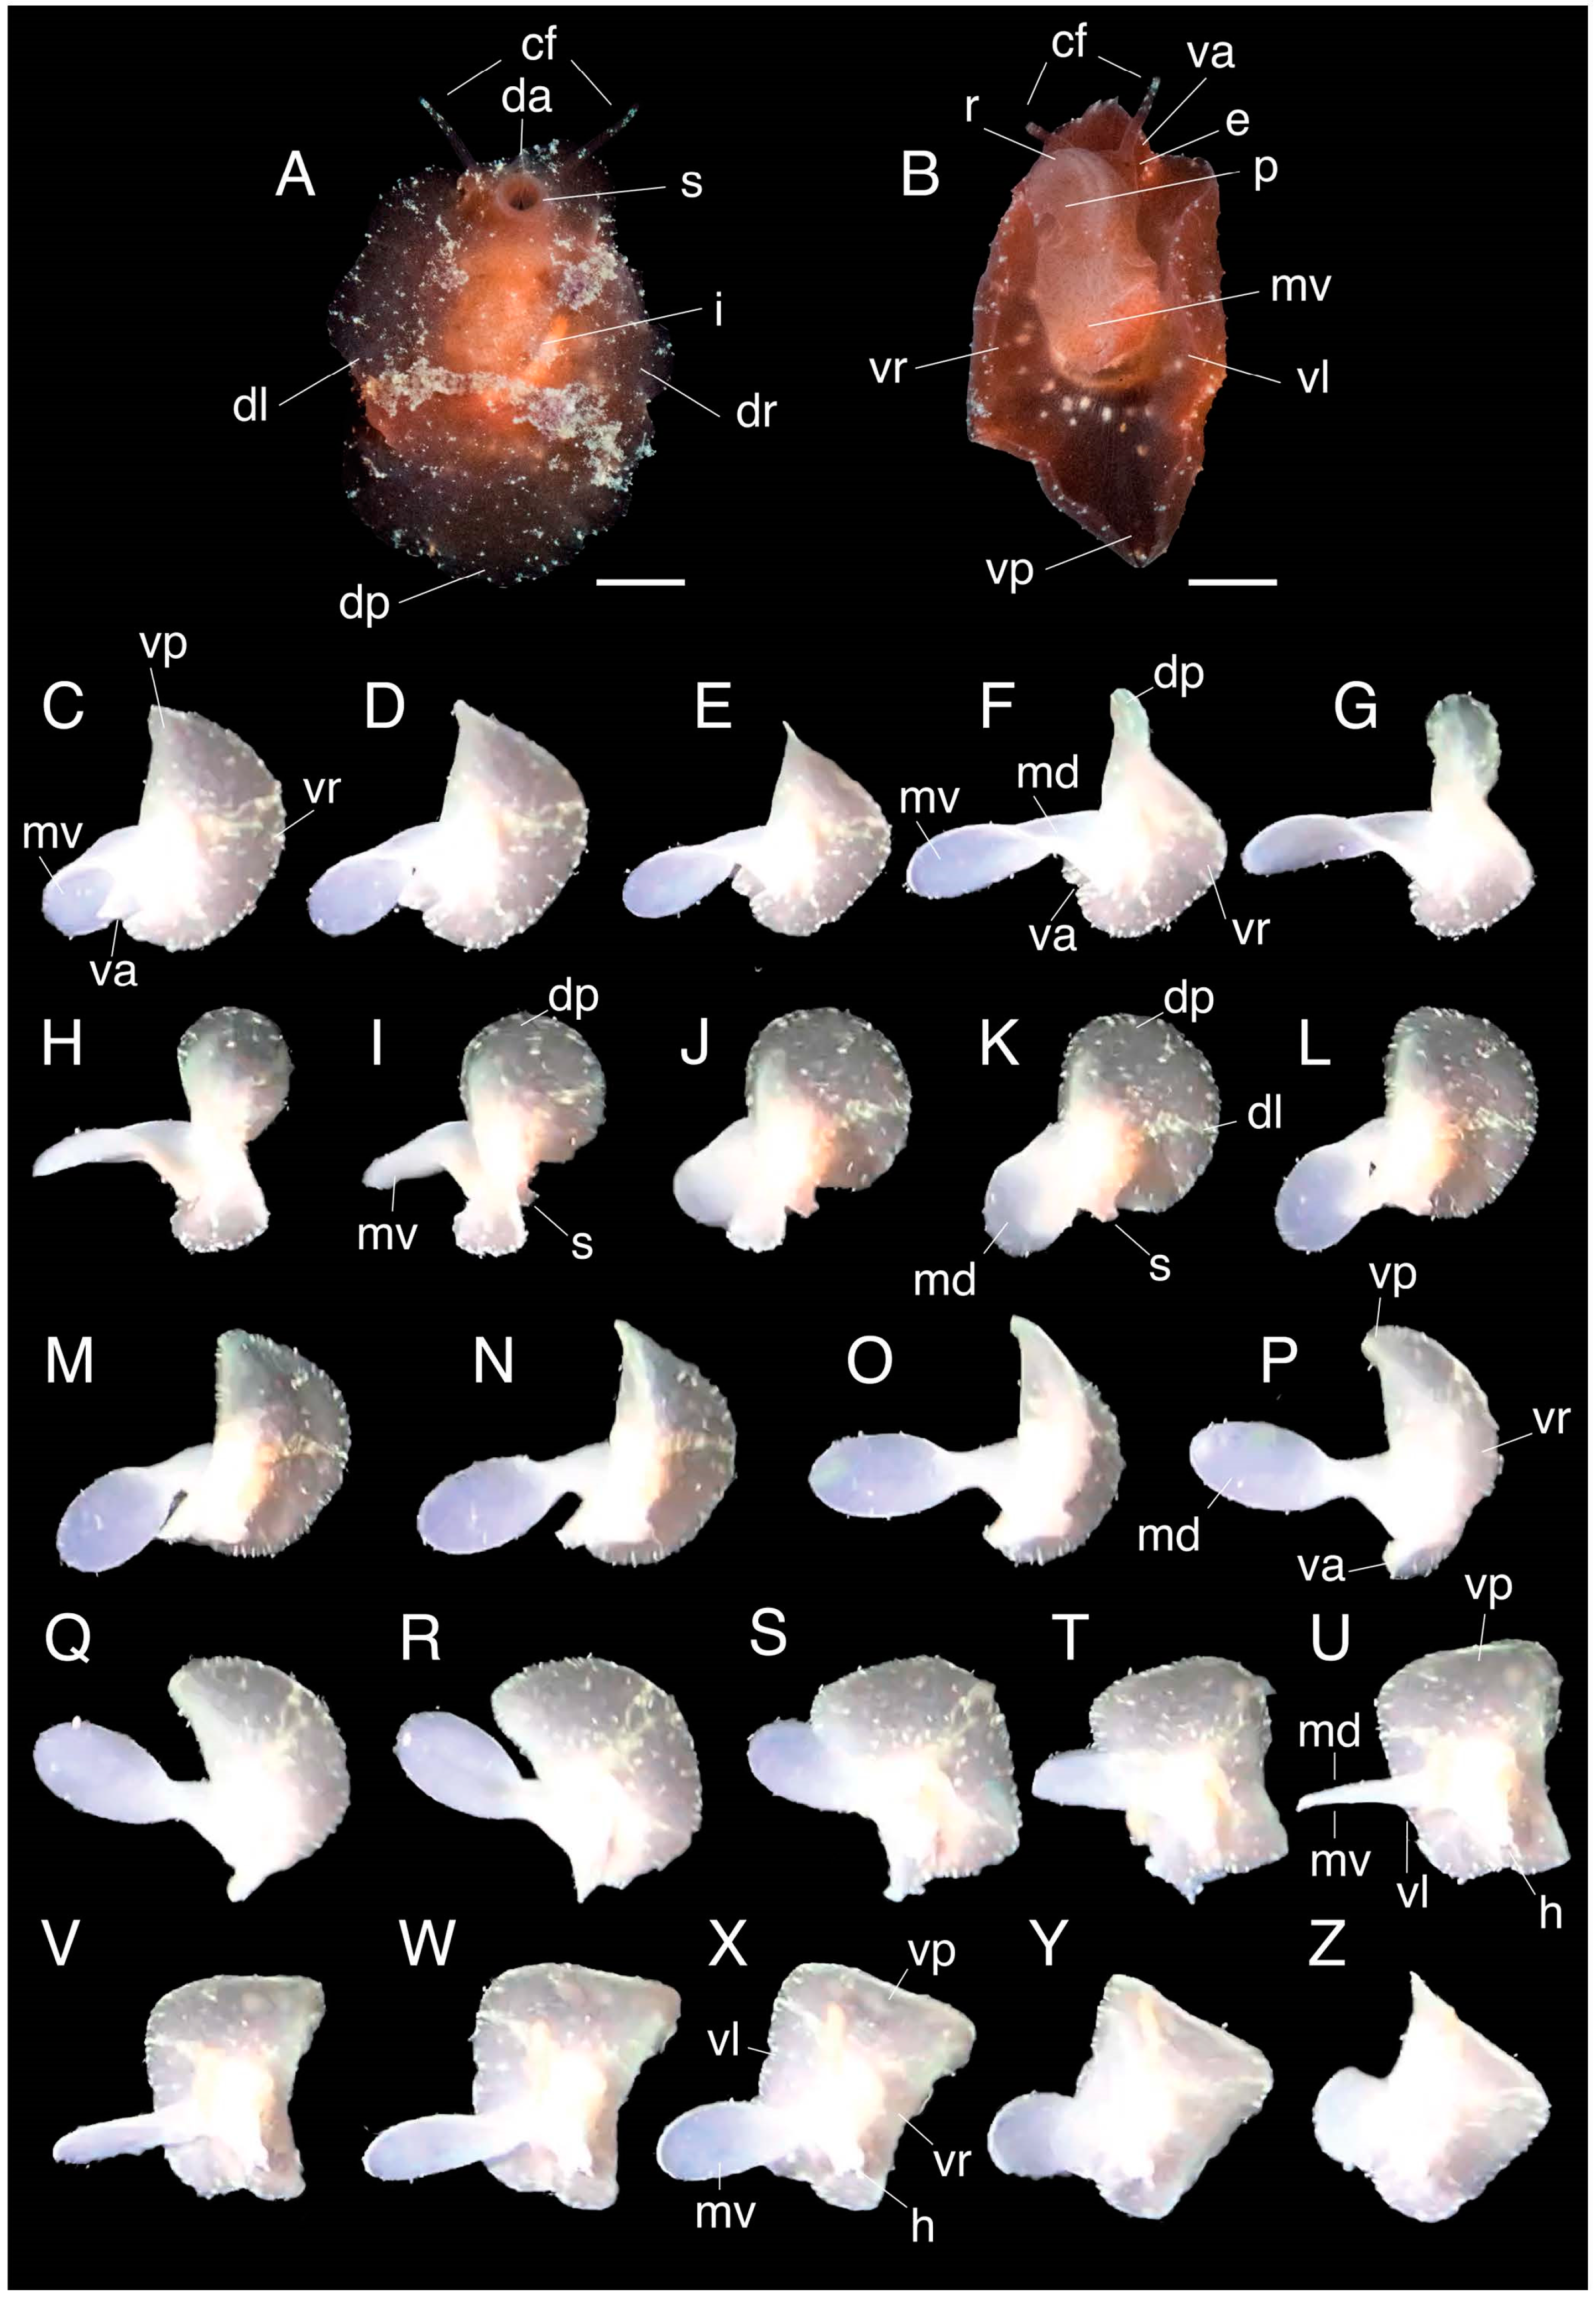
A specimen of the genus Marsenia sp. Oken, 1823 (Velutinidae: Lamellariinae), was filmed while swimming by J.B. during a night dive in Bayu Is. (New Caledonia, <1 m depth, approximately three hours after sunset; locality details in Supplementary Material Table S1), during the scientific expedition “ABC Poum 2023”, organized by the Muséum national d’Histoire naturelle, Paris (MNHN). The specimen was then collected, photographed alive in the lab (Figure 1A,B), and preserved in 96% ethanol. Considering the high morphological plasticity of velutinids that hampers their identification, a molecular approach was used to identify this specimen at the species level. DNA was isolated from a tissue clip of the foot using a “salting-out” protocol [4], and the cytochrome oxidase subunit I mitochondrial marker (COI) was amplified by PCR and sequenced (following [7]). A molecular dataset was created, including 17 other COI sequences of velutinids retrieved from GenBank (Supplementary Material Table S1). COI pairwise genetic distances were calculated using the Kimura two-parameter model, and a Bayesian inference phylogenetic tree was produced (following [8]). The collected snail clustered in a statistically supported clade (posterior probability = 1), including other specimens identified by Fassio et al. [4] as Marsenia cf. gemma Bergh, 1875 (Supplementary Material Figure S1). The intraspecific range of COI distances between individuals clustered in the clade of Marsenia cf. gemma (0–1%; Supplementary Material Table S2) and the interspecific range calculated with the other specimens of the dataset (8.2–19.57%; Supplementary Material Table S2) further supported the identification of the collected specimen as Marsenia cf. gemma.
Figure 1.
Marsenia cf. gemma MNHN-IM-2019-30080 (New Caledonia). (A), dorsal side; (B), ventral side, showing the snail head with cephalic tentacles and the contracted foot. (C–Z), frames of the video showing the movement of the velutinid while swimming in the water column. The complete foot movement sown in (C–X) lasted 0.683 s. Scale bars: (A,B), 1 mm. cf, cephalic tentacles; da, dorsal anterior side of the mantle; dl, dorsal left side of the mantle; dp, dorsal posterior side of the mantle; dr, dorsal right side of the mantle; e, eye; h, head; i, internal organs visible through the mantle; mv, ventral side of the metapodium; md, dorsal side of the metapodium; p, propodium; r, double rim of the propodium; s, siphon; va, ventral anterior side of the mantle; vl, ventral left side of the mantle; vp, ventral posterior side of the mantle; vr, ventral right side of the mantle.
The snail body is entirely covered on the dorsal side by a flat and thin mantle, mostly orange in color, with white and pink dots, streaks, and patches (Figure 1A). The mantle is relatively transparent, and in its central part, the internal organs (enclosed in a vestigial, transparent, internal shell) can be glimpsed (Figure 1A). On the anterior part, the mantle is folded, forming an inhalant siphon (Figure 1A). On the ventral side (Figure 1B), the head has a pair of elongated cephalic tentacles, each with an eye at the base, on the outer side. The foot can be divided into a front part, the propodium (approximately the anterior third of it), showing a double rim at the upper extremity, and a rear part, the metapodium, detached from the rest of the body for most of its length (Figure 1B).
As observed in the video (Supplementary Material Video S1 and frame sequence in Figure 1C–Z), the velutinid is actively swimming upward in the water column, head down. The mantle is extended and tense, incurved backwards on both its right and left sides, and the metapodium (the rear part of the foot placed on the ventral side of the animal) is extended, flatted, and used as a paddle. The metapodium is waved for propulsion following a ∞-shaped curve: upper left—down left—center—upper right—down right—center. During the downwards movement, the ventral side of the metapodium is always facing down. The movement sequence starts with the metapodium curved on the left side of the snail (Figure 1C), note that the snail head is always down), paddling down using the ventral side. Then, the metapodium changes inclination and moves first to the center of the snail, with the ventral side facing the right side of the animal (Figure 1F), then to the right side, with the ventral side facing down (Figure 1I). At this point, the metapodium moves downwards, with the ventral side pushing the water (Figure 1J–K). Then, the metapodium changes inclination again and moves back to the center of the snail, with the ventral side this time facing the left part of the animal (Figure 1P). After that, the metapodium moves back to the left side of the snail, changing inclination to have the ventral side facing down (Figure 1U), and pushes downwards (Figure 1V–X). Then, the full movement is repeated in a loop. During the first 16 s of the video, 23 complete foot movements were observed and timed, with each loop taking 0.633 s to be completed, on average (making approximately 38 loops per minute).
At least one other specimen of Marsenia sp. was observed in the aquarium extending and flattening the metapodium, almost doubling its length, and moving it from the right side to the left and back for several seconds as a response to being turned upside down (G.F. personal observation). However, to our best knowledge, this is the first time that a swimming behavior is observed in an adult velutinid. This may represent a voluntary behavior, for example, an escape response from predators, a dispersal strategy to increase the chance of reaching a suitable area for feeding and/or reproducing (velutinids feed and lay eggs on ascidians and are mostly gonochoristic [4,5]), or a survival response when the animal finds itself detached from the substratum and adrift in the water column. The snail was already swimming when spotted by divers, so it cannot be determined whether this behavior was elicited by the light of divers’ flashlights.
Considering this single record, it is hard to hypothesize if this ability is limited to this species or if it is more ubiquitous in the subfamily Lamellariinae d’Orbigny, 1841, or in the family Velutinidae. However, looking at the morphological characters that may facilitate Marsenia cf. gemma to swim (a thin, weakly calcified, ear-shaped, internal shell; a flat and smooth mantle; a muscular and flat foot) these are shared with several other species of the same genus and with other lamellariin genera, such as Lamellaria Montagu, 1816, and Djiboutia Vayssière, 1912. Regarding the fact that this observation was made during a night dive, velutinids are not known to be specifically nocturnal animals, so it can be supposed that this behavior is not strictly limited to nighttime.
Because this ability, quite unexpected for the group, has been observed only once so far, several questions still remain unanswered, such as why a velutinid is induced to swim or how common this behavior is within the family. However, it has changed our perspective toward the biology of this group, previously thought to have a sedentary and benthic adult life, but now shown to also possess the ability to swim.
Supplementary Materials
The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/d16010040/s1. Table S1: sequences used for molecular analysis (including voucher codes, sampling localities, and GenBank accession numbers); Table S2: pairwise COI genetic distances calculated between velutinid specimens; Figure S1: Bayesian Inference tree of the COI velutinid dataset; Video S1: underwater video of the swimming Marsenia cf. gemma.
Author Contributions
Conceptualization, G.F.; Formal Analysis, G.F.; Investigation, G.F. and J.B.; Writing—Original Draft Preparation, G.F.; Writing—Review and Editing, G.F. and J.B.; Visualization, G.F.; Funding Acquisition, G.F. All authors have read and agreed to the published version of the manuscript.
Funding
This research was partially funded by Sapienza University of Rome SEED PNR 2021 grant n° B89J21032850001 to G.F.
Institutional Review Board Statement
Not applicable.
Data Availability Statement
COI sequence was deposited at GenBank (accession number: OR933637).
Acknowledgments
The specimen was collected under the auspices of the Our Planet Reviewed programme at the MNHN during the Atlas de la Biodiversité Communale (ABC) of the commune de Poum, PI Dominique Fleurot, with funding from the Office Français de la Biodiversité (OFB) and Fondation Gingko. The field work operated under Autorisation simplifiée 609011-23/2023/DEPART/JJC issued 3 April 2023 by Jean-Jerome Cassan, Service Impact Environnemental et Conservation, Province Nord. Special thanks go to Philippe Bouchet (MNHN) for the opportunity to work on New Caledonia material, to Barbara Buge (MNHN) for the precious help with MNHN vouchers, and to Giacomo Chiappa (Sapienza University of Rome) for the help with molecular sequences. Two anonymous reviewers are thanked for useful comments that helped to implement this paper.
Conflicts of Interest
The authors declare no conflicts of interest.
References
- Farmer, W.M. Swimming gastropods (Opisthobranchia and Prosobranchia). Veliger 1970, 13, 73–89. [Google Scholar]
- Ellingson, R.A.; Krug, P.J. Reduced genetic diversity and increased reproductive isolation follow population-level loss of larval dispersal in a marine gastropod. Evolution 2016, 70, 18–37. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Modica, M.V.; Russini, V.; Fassio, G.; Oliverio, M. Do larval types affect genetic connectivity at sea? Testing hypothesis in two sibling marine gastropods with contrasting larval development. Mar. Environ. Res. 2017, 127, 92–101. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fassio, G.; Stefani, M.; Russini, V.; Buge, B.; Bouchet, P.; Treneman, N.; Malaquias, M.A.E.; Schiaparelli, S.; Modica, M.V.; Oliverio, M. Neither slugs nor snails: A molecular reappraisal of the gastropod family Velutinidae. Zool. J. Linn. Soc. 2023, 197, 924–964. [Google Scholar] [CrossRef] [Scilit]
- Wilson, B. Superfamily Velutinoidea. In Mollusca: The Southern Synthesis. Fauna of Australia; Beesley, P.L., Ross, G.J.B., Wells, A., Eds.; Part B.; CSIRO Publishing: Melbourne, Australia, 1998; Volume 5, pp. 786–790. [Google Scholar]
- Fassio, G.; Modica, M.V.; Alvaro, M.C.; Buge, B.; Salvi, D.; Oliverio, M.; Schiaparelli, S. An Antarctic flock under the Thorson’s rule: Diversity and larval development of Antarctic Velutinidae (Mollusca: Gastropoda). Mol. Phylogenet. Evol. 2019, 132, 1–13. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fassio, G.; Bouchet, P.; Lozouet, P.; Modica, M.V.; Russini, V.; Schiaparelli, S.; Oliverio, M. Becoming a limpet: An ‘intermittent limpetization’ process driven by host features in the kleptoparasitic gastropod family Capulidae. Mol. Phylogenet. Evol. 2021, 155, 107014. [Google Scholar] [CrossRef] [Scilit]
- Fassio, G.; Modica, M.V.; Alvaro, M.C.; Schiaparelli, S.; Oliverio, M. Developmental trade-offs in Southern Ocean mollusc kleptoparasitic species. Hydrobiologia 2015, 761, 121–141. [Google Scholar] [CrossRef] [Scilit]
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2024 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).