


Abstract
The aim of the study was to investigate the effect of vegetation cover and height on soil and plant nutrients across managed and unmanaged agricultural land in a temperate climate. Fresh soil and vegetation samples were collected during the years 2023 and 2024 from 125 different land parcels in the southwest of the UK. Land was either managed for grazing and/or feed production or not managed for agricultural use, and had a range of grass, crop, legume, herb, and flower species. A linear mixed model was used to assess the effect of vegetation height (in cm) and cover (tonnes of dry matter per hectare) on soil and plant nutrients. The results showed plant dry matter (DM) digestibility, acid detergent fibre (ADF), water-soluble carbohydrate, and oil contents increased with vegetation height, and soil DM and neutral detergent fibre (NDF) decreased with vegetation height. The ratio of soil-to-plant OM reduced and ADF increased with increasing vegetation cover. Interactions between vegetation height and cover (i.e., density) were found for the ratio of soil-to-plant OM, ADF, NDF, DM, DM digestibility, oil, water-soluble carbohydrate, and crude protein nutrients. Measuring the interaction between soil and plant properties showed soil OM stocks increased and soil pH decreased with increased vegetation cover across agricultural land.
1. Introduction
Sustainable agricultural productivity and ecosystem preservation can be improved by understanding vegetation cover interactions with soil nutrients such as organic matter and pH [1]. Information on changes in vegetation cover and height are relevant in determining soil health because these properties influence the level of added soil organic matter and nutrients [2]. Soil nutrients are utilised by plants and degraded plant cover is important for soil nutrient availability, thus indicating the existence of a symbiotic relationship between soil and plant cover [3]. For informed decision making and optimum yield of agricultural crops and pastures, plant and soil interactions require proper evaluations to understand the effect of land management changes. Root biomass and plant residues are the main sources of soil organic matter and help support the structure of the soil [4]. Soil is productive if it has good structure and good water-holding and nutrient retention capacity, and these can be improved by high vegetation cover associated with adequate organic matter supply in the soil [5]. Soil pH stability is promoted by high vegetation cover, which helps buffer against the process of acidification, though stability can be affected by changes in plant species composition and their associated decomposition rates [6].
The height of vegetation is a suitable measure for estimating the maturity of above-ground plant biomass. Maturity of vegetation is associated with taller plants with lower quality and digestibility due to increased fibre proportions such as high lignin and cellulose [7,8]. Increased plant height may also result in the dilution of plant nutrients in nutrient-rich tissues, such as leaves, thereby lowering the contents of crude protein and oil found in leaves [9]. In livestock grazing, productivity of pastures is measured by the quantity and quality of forage, with forage yield and maturity being managed to ensure nutrient richness [10]. Despite these well-established links, many previous studies have focused on either vegetation or soil properties in isolation, often using destructive and time-intensive laboratory methods such as loss on ignition for organic matter content analysis and the pipette or hydrometer methods for particle size–texture analysis. The emergence of real-time NIRS offers a transformative approach to analysing whole samples of fresh organic material in the field. The use of NIRS enables frequent, low-cost, and non-destructive measurement of common soil and plant nutrients to allow exploration of relationships [10,11]. This approach is helping to inform agricultural land-use decision making. For example, a managed and fertilised grassland used for grazing will typically experience changes associated with animal and land management, which will subsequently shape the composition of plant species and the nutrient characteristics of soil and plant biomass [12,13]. On the other hand, unmanaged or semi-natural land may be abundant in diverse communities of plant species and thereby become more resilient with high nutrient-retaining capacity in the long term [14,15]. These differences highlight the importance of comparing vegetation structure and soil properties across land-use gradients to inform regenerative and climate-smart agricultural strategies. Grasslands, which dominate much of the United Kingdom (UK) and global agricultural landscape, are of particular interest in this context. They not only provide a critical forage base for livestock but also offer opportunities to enhance biodiversity, carbon sequestration, and water regulation when managed sustainably [16,17].
Generally, UK grassland systems have prioritised productivity through monocultures of high-yielding species like perennial ryegrass (Lolium perenne), selected for traits such as high dry matter yield, crude protein, and sugar content [9,18]. However, this productivity focus has increasingly been balanced with environmental concerns, including reducing synthetic fertiliser dependency, man-made inputs, chemicals, and organic fertilisers and improving drought resilience [19]. Recent research supports the use of multispecies swards with grasses, legumes, herbs, and flowering species to improve both forage productivity and soil health [20]. These mixed systems are known to promote complementary resource use, enhance plant nutrient uptake, and increase resilience to climatic stress [8,15]. Moreover, such diversity can increase root exudation and microbial activity, leading to improved nutrient cycling and soil carbon retention [3]. This study contributes to this growing body of knowledge by assessing how vegetation cover and height affect key soil and plant chemical properties using real-time NIRS across a range of managed and unmanaged land in the UK. By analysing both the independent and interactive effects of vegetation cover and height, it offers new insights into how plant–soil responses function in temperate agroecosystems. The findings are relevant not only for pasture management and livestock production but also for crop production and broader goals related to soil conservation, biodiversity, and climate change mitigation.
The objective of this study was to investigate the effect of vegetation height and cover on soil and plant nutrients across managed and unmanaged agricultural land in a temperate climate.
2. Materials and Methods
2.1. Study Area and Field Data
The study was conducted across 125 established fields and grassland plots (28 arable crops, 41 temporary ley grasslands, and 56 permanent grasslands) across nine farms in the southwest of England (51.91° N, −2.31° W to 51.89° N, −1.84° W, 41 m a.s.l) between March 2023 and August 2024. Five farms were in the Severn Vale region, and four farms were in the Cotswold National Landscape. The fields studied were managed for agricultural production, whereas grassland plots (~6 m2) were left undisturbed and not used for agricultural production. The grassland plots consisted of 4 randomised blocks of 6 plots (~6 m2) with either herbal ley, mustard/radish cover crop, wildflowers, ryegrass/clover mix, or native grass species. The fields and plots provided diversity in terms of plant species composition, stage of growth, age, and land use. The soil in the region is predominantly clay loam. The region studied has a temperate climate and is dominated by grassland. The ambient temperature and rainfall were recorded by a local Met Office weather station. The average daily temperature was similar across study years (Table 1) and the average monthly rainfall was slightly higher in 2024 compared to 2023.
Table 1.
Average daily temperature and monthly rainfall during the study period.
2.2. Sample and Field Data Collection
A total of 803 soil and 803 fresh vegetation samples were collected. Soil and plant samples were collected at the same time from the same location and within a 30 cm diameter wire ring (0.1 m2) randomly placed on the ground. In the plots, two random samples were taken within the plot, whereas in each field, five samples were obtained after walking in a W-pattern across the field.
2.2.1. Plant Measurements
A rising plate meter (F400; Farmworks Precision Farming Systems Ltd., Feilding, New Zealand) was used to measure vegetation height in centimetres [10]. The vegetation height of each field and plot was estimated from the average ‘spot’ measurements when walking the W-pattern across the area sampled. Each time the rising plate meter was lowered into the sward, it measured the compressed plant height, with each click of the meter representing ½ cm in height.
Plant samples were taken from each point of the ‘W’ pattern across the area sampled using a 36 cm diameter wire ring (0.1 m2 and 1 hectare is 10,000 m2). Samples were cut within the ring to ground level and placed in a labelled bag. Collected samples were transferred to a fridge as soon as possible (4 °C) for further analysis. The fresh weight (FW) (in grams) of plant material within the cut area was multiplied by 10 to estimate the FW cover in tonnes FW/ha based on the area of the sampling ring (i.e., 1 hectare (ha) = 10,000 m2). The FW cover value was then multiplied by the percentage of DM obtained by nutrient analysis to derive the DM cover in tonnes DM/ha. The average FW and DM cover was divided by the vegetation height to derive the density of vegetation in t FW/ha/cm and t DM/ha/cm.
Plant nutrients of dry matter (DM), crude protein, acid detergent fibre (ADF), neutral detergent fibre (NDF), water-soluble carbohydrates, ash, dry matter digestibility (DMD), and oil (all in g/kg DM) were measured by scanning collected fresh samples using a mobile NIRS plant scanner (NIR4; Aunir, Towcester, UK). The NIRS scanner consists of a spectrum of infrared energy reflected from the sample illuminated during scanning. It conducts a pre-scan calibration with a standard white plate before scanning the sample, with five replicate scans performed per sample. Each of the fresh plant samples collected were placed in a bowl. The NIRS plant scanning head was placed on the plant material in the bowl, pressing down to ensure no external light interference. When scanning was completed, the resulting nutrient analysis was automatically uploaded to cloud storage via a tablet.
2.2.2. Soil Measurements
Soil samples were taken to 30 cm depth within the wire ring [10]. Soil samples were collected using a 2 cm diameter soil corer and nutrient analysis was carried out using a mobile NIRS soil scanner (Agrocares, series-E; Wageningen, The Netherlands). The mode of analysis of soil samples using the soil scanner is very similar to the plant scanner described above. Each of the fresh soil samples were placed in a small dish, which helped prevent external light interference. The scanner head was placed on the soil in the dish after levelling the soil and after conducting a pre-scan calibration against a white plate, and the scanner performed four replicate scans per sample. When scanning was completed, the resulting nutrient analysis was automatically uploaded to cloud storage via a tablet.
Soil nutrients of organic matter (OM); total nitrogen (N; both g/kg and t/ha); clay; moisture (both %); pH; and ratios of organic carbon to nitrogen, organic matter to clay, and organic matter to plant organic matter contents were determined. Dry soil content (in grams) was divided by soil volume (in cm3) to estimate bulk density (g/cm3) and used to estimate organic matter and total nitrogen stock (t/ha = [10,000 × soil depth cm/100 × bulk density g/cm3 × OM or N g/kg]/1000).
2.3. Statistical Analysis
Data were analysed in SPSS (IBM SPSS Statistics for Windows, Version 29.0; Armonk, NY, USA). A total of 222 average values for sampled areas during the study period were used for the analysis. A linear mixed model (Equation (1)) was used to assess the effect of vegetation cover and height on soil and plant nutrients, with the random effect of farm included as
where Yij is a dependent plant or soil nutrient; µ = intercept; b1H = linear regression of Y on vegetation height in cm; b2V = linear regression of Y on vegetation cover in t DM/ha; F = random effect of farm (i = 1 to 9); M = random effect of month (j = 1 to 12); and e = random error term. Significance was attributed at p < 0.05.
Yij = µ + b1H × b2V + Fi × Mj + eij
3. Results
The plant species across fields and plots were identified and recorded during plant sampling. A wide range of plant species were identified and included: wheat (Triticum aestivum), barley (Hordeum vulgare), perennial ryegrass and hybrids (Lolium perenne), timothy (Phleum pratense), Yorkshire fog (Holcus lanatus), cocksfoot (Dactylis glomerata), common bent (Agrostis capillaris), oat grass (Arrhenatherum elatius), meadow grass (Poa annua), sweet vernal grass (Anthoxanthum odoratum), soft brome (Bromus hordeaceus), crested dogstail (Cynosurus cristatus), chicory (Cichorium intybus), plantain (Plantago lanceolate), red clover (Trifolium pratense), alsike clover (Trifolium hybridum), white clover (Trifolium repens), sainfoin (Onobrychis vicifolia), burnet (Sanguisorba minor), mustard (Sinapsis alba), raddish (Raphanus sativus), knapweed (Centaurea nigra), field poppy (Papaver rhoeas), yarrow (Achillea millefolium), bindweed (Convolvulus arvensis), ox-eye daisy (Leucanthemum vulgare), broad-leaved dock (Rumex obtusifolius), common dandelion (Taraxacum officinale), creeping buttercup (Ranunculus repens), and heal-all (Punella vulgaris).
Across the areas studied, there was considerable variability in vegetation height, cover (fresh and dry matter), and density (fresh and dry matter), with coefficients of variation ranging >70%; Table 2). All plant nutrients studied showed variability. The soil organic matter content was the most variable soil nutrient (>40%; Table 2).
Table 2.
Average vegetation cover, vegetation nutrients, and soil nutrients across samples collected.
3.1. Effect of Vegetation Cover and Height on Plant Nutrients
The ADF, water-soluble carbohydrate, oil (all p < 0.001), and DM digestibility (p < 0.01) content of vegetation increased with taller vegetation, and dry matter (p < 0.001) and NDF (p < 0.05) reduced with taller vegetation (Table 3). The ADF content (p < 0.05) increased and DM content reduced (p < 0.05) with higher vegetation cover. There was an interaction between vegetation height and cover for DM, crude protein, ADF, NDF, DMD, oil (all p < 0.001), and water-soluble carbohydrate (p < 0.05). There was no effect of vegetation height or cover on ash content.
Table 3.
Effect of vegetation cover and height on plant nutrients.
3.2. Effect of Vegetation Cover and Height on Soil Nutrients
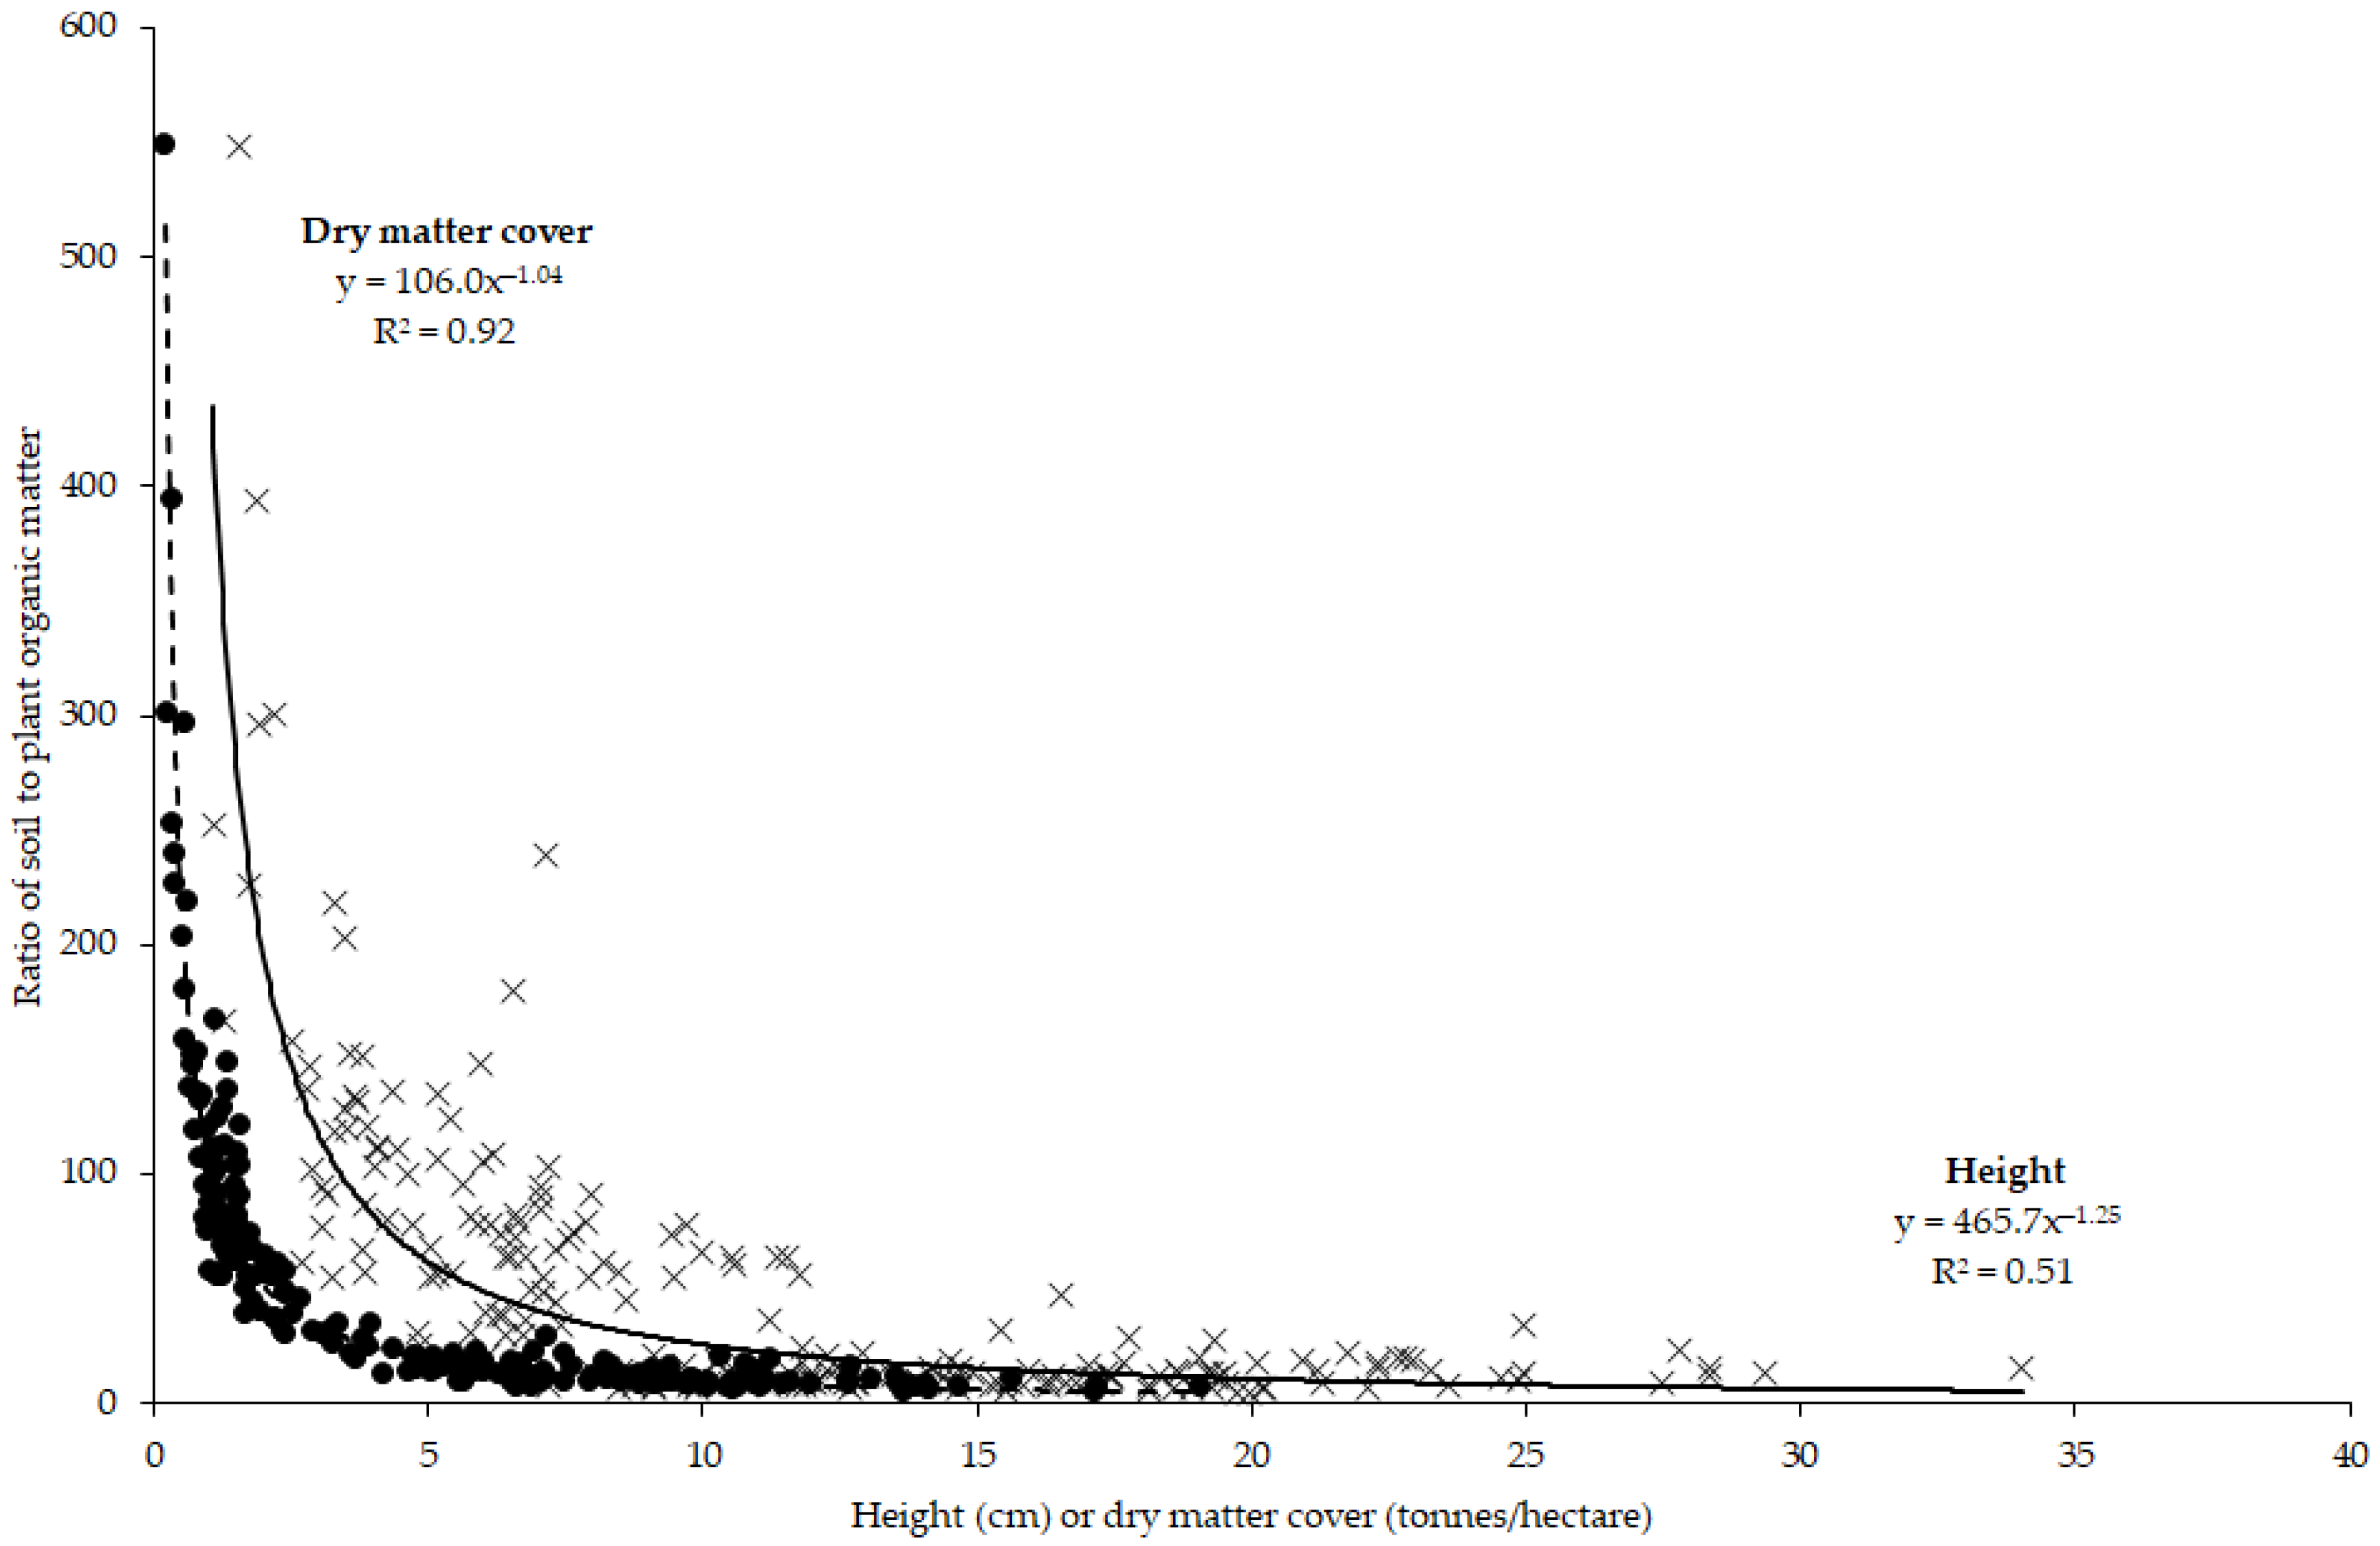
The ratio of soil OM to plant OM reduced with increased vegetation height and cover (p < 0.001; Table 4). Significant soil-to-plant OM ratio effects against height, dry matter cover, and density (height × cover) were observed (p < 0.001; Figure 1). The OM stock increased with increased vegetation cover and pH reduced with increased vegetation cover (both p < 0.05). There was no interaction between vegetation height and cover (p = 0.145 for OM; p = 0.051 for pH).
Table 4.
Effect of vegetation cover and height on soil nutrients.
Figure 1.
Change in soil-to-plant organic matter ratio with plant height (crosses and solid line) and dry matter cover (dots and dashed line). Line of best fit shown.
4. Discussion
Denser cover means more competition among plants (for light and nutrients), which often leads to plants producing more supportive or fibrous parts (stems, etc.) that are less nutrient-dense. For example, protein, water-soluble carbohydrates, digestibility, and oil reduced with increasing density (interaction between height and cover) in the current study. Several studies have established that increasing plant density leads to stronger competition for light and nutrients, causing plants to put more of their growth into stems and support structures instead of tissues that actively carry out metabolism. It has been confirmed in previous research that, under competitive conditions, plants increase allocation to stems and structural tissues to enhance growth and light capture, resulting in reduced nitrogen and soluble carbohydrate concentration in leaves [21]. This explains why dense grass swards consistently exhibited lower crude protein and digestibility in previous studies due to dilution effects caused by increased structural biomass [22]. Increased shading in dense stands stimulates lignification, which directly reduces digestibility and energy availability [23]. Research has shown that when the cover is dense, there is more plant material going back into the soil from plant litter and roots, so soil OM increases [3]. The NDF of plants is known to increase with stem proportion and maturity, as found in the current study [24]. Plant fibre content increases more rapidly when plants grow taller under competitive conditions, as internode elongation and secondary cell wall development are accelerated [25,26]. It could be generalised from the current study findings that the interaction between height and cover supports the idea that height alone does not drive fibre accumulation; rather, it is height under competition that increases NDF and reinforces the importance of structural context.
Taller vegetation was associated with ADF and higher DM digestibility. This supports other research findings which show that as plants mature, this often correlates with height and fibre often increases, but digestibility may still be reasonably high depending on the species and whether it is grazed or used for forage production [7]. In previous studies, it was found that increased ADF with plant height does not always cause proportional declines in digestibility, especially when tall vegetation remains leaf-rich [27]. Other literature reported that digestibility depends on the balance between lignin concentration and leaf-to-stem ratio, not height alone [25]. Taller species may maintain relatively high digestibility if growth is rapid and tissues are less lignified [28,29]. These relate to this study, as it is shown in this study that taller plants had higher ADF but were still digestible, showing that forage quality depends more on plant traits and tissue composition than on plant height alone. There was a significant effect of vegetation height on several plant nutrients despite the limited effect on soil nutrients in the present study. Research shows that this effect implies that the plant invests in height and structure, while nutritive elements like protein and digestibility decline as fibre increases [30]. The reduction in soil-to-plant OM ratio with increasing cover aligns with the soil research findings and further supports the conclusion that high vegetation density accelerates organic inputs to the soil, potentially improving soil carbon storage and fertility [3]. Perennial vegetation cover moves more carbon from plant biomass into the soil, reducing the amount of organic matter kept in living plant tissue [28,31]. This process is referred to in other research as a key mechanism of soil carbon sequestration in grasslands [32,33]. In tall vegetation or high cover, the soil-to-plant OM ratio starts to plateau at about 10:1 (Figure 1).
Research on grasslands has shown that good vegetation covers increased soil organic content fairly and rapidly [34], thus, aligning with this study’s findings of high soil OM with increasing vegetation cover. Also, this finding is supported by a previous study which showed that good cover and diverse species lead to improved soil physicochemical properties (including organic matter) and better nutrient status in many grassland soils [7]. However, it should be noted that other research has indicated that taller species may be dependent on the plant types and their growth rate; for example, legumes or fast-growing grasses both have high structural development and elevated metabolic rates, which translates into higher energy content and increased height [8]. Research reports that grasslands with higher biomass production and ground cover accumulate soil organic carbon faster due to greater litter and root inputs [35]. It is also established that dense vegetation enhances soil OM stabilisation by increasing particulate organic matter and aggregate formation [36]. Increased vegetation cover shifts carbon from plant biomass into soil pools, particularly in perennial grasslands [37]. Thus, the observation of increased soil OM with increasing cover in this study confirms that dense vegetation enhances carbon inputs through both above- and below-ground biomass, improving soil carbon storage. Some plant communities with greater height may reflect more competitive species that invest in both structure and photosynthetic capacity, balancing fibre content with nutritional value. The reduction in NDF and DM can also be dependent on plant-type differences in terms of physiology and growth rate. For example, it is indicated in other literature that in some species, taller vegetation may be composed of tissues with higher water content and lower cell wall complexity, possibly reflecting a shift toward leafier growth or species with less lignified biomass [38]. The decrease in oil content could result from a lower prevalence of oil-rich plants in taller stands dominated by grass.
Vegetation cover had a significant effect on specific soil properties of OM stock and pH in the current study. Other studies, however, have shown that increased plant biomass inputs promote the addition of organic carbon to the soil [2,5]. This study finding aligns with research studies that show that denser vegetation increases plant residues and root biomass in land and therefore promotes the addition of organic compounds to the soil, enhances microbial activity, and contributes to humus formation [2,5]. It has been shown from other research that this will subsequently lead to greater stabilisation of organic carbon, maintenance of fertility, water retention, and carbon sequestration in the soil [39]. The observed decline in soil pH with increasing vegetation cover may be explained by several mechanisms. Firstly, research shows that decomposition of organic material often produces organic acids, which acidify the soil microenvironment [40]. Secondly, research indicates that denser plant cover may promote specific microbial communities that can process organic matter through pathways that generate acidic byproducts, such as nitrification or fungal decomposition [2,5]. Additionally, from other research findings, it could be derived that competition for cations like calcium, magnesium, and potassium are common in dense vegetation and can result in base cation depletion, thereby lowering pH further [4]. This dynamic is particularly relevant in temperate regions like the UK, where relatively high rainfall can exacerbate leaching of base cations in high-biomass systems. Increasing organic matter inputs has been reported to lower soil pH due to organic acid production during decomposition [41]. It has also been demonstrated that high plant uptake of base cations in dense vegetation can lead to soil acidification [42]. The pH declines with increasing cover observed in this study are consistent with organic acid formation, microbial activity, and base cation depletion, which are common in high-biomass grasslands [33,43].
In the current study, there were no significant effects of vegetation height on soil nutrients, except the ratio of soil-to-plant OM. This suggests that vegetation height, and interaction with vegetation cover, plays a limited role in the soil nutrients studied. This result aligns with other research findings that show that the addition of major plant-derived inputs to soil, e.g., plant residues, root turnover, and exudates takes place at or below the soil surface and is therefore more closely related to vegetation cover than height [3,33,44]. In recent research observations in the UK, less-disturbed cropland soil with more vegetation cover showed increased soil organic carbon, after many years of decline [45]. Also, another study reported a rapid increase in soil organic carbon and total nitrogen where vegetation was restored in predominant grassland; vegetation height did not have much effect on soil properties like pH or organic matter [34]. This suggests that plant density or cover determines soil processes, rather than vegetation height. This aligns with the findings from previous grassland studies in the UK which showed that less intensively managed grasslands had better vegetation cover and density, resulting in increased soil nutrients, such as soil carbon and nitrogen, than intensively managed land [45]. Soil nutrient dynamics are more strongly linked to root biomass and litter input than above-ground height [31,46]. In grassland research, it should be noted that plant height has been reported to have minimal effect on soil carbon and nitrogen compared to vegetation cover and management [47,48]. In this study, it has been confirmed that soil nutrient processes respond primarily to vegetation cover and below-ground inputs rather than plant height.
One of the most significant findings of this study is the interaction of vegetation height and cover and their effects on plant nutrients such as ADF, NDF, DMD, oil, water-soluble carbohydrate, protein, and soil-to-plant OM ratio. These nutrient changes indicate that the interaction between vegetation cover and height (structure) has a significant effect on plant quality and as such, vegetation cover cannot be considered separately from plant height because dense or sparse vegetation cover will affect the forage quality and nutritional status of a tall plant differently. It can therefore be suggested that, in sparse areas, taller plants may be younger and more palatable, whereas in dense stands, taller plants might be older and more fibrous, reducing digestibility. This is supported by previous research findings which showed that the impact of plant height on digestibility may be stronger or weaker depending on how dense the sward is. A previous study showed a similar interaction where vegetation cover and species phenology together under different environmental or management conditions affected plant digestibility and protein content more than any single factor alone [6]. Similarly, high protein content may occur in short but dense swards dominated by legumes, whereas tall and sparse vegetation might have lower protein but higher fibre [8]. Forage quality can depend on sward density and phenological stage [22,49]. Digestibility and protein content have been reported to be governed by combined effects of canopy structure, species composition, and competition [27,50]. Dense tall grass swards tend to be more fibrous, while tall sparse stands may retain higher nutritional value [51]. It is further confirmed in this study that vegetation structure must be interpreted multidimensionally; height and cover jointly determine plant age, fibre accumulation, and nutrient concentration. These interactive effects highlight the complex state of plant and soil interactions in real-world ecosystems. Vegetation structure is shaped by numerous factors including species composition, land-use history, grazing or mowing intensity, and microclimatic conditions [13]. Therefore, managing optimal forage quality and soil health requires a detailed understanding of how these variables interact. It has been established in other research that legumes maintain higher protein and digestibility even at higher densities due to nitrogen fixation [52]. It has also been reported that fast-growing species may be both tall and nutrient-rich due to high photosynthetic capacity [21]. Species effects explain variability in NDF, DM, and oil content across height and cover gradients [26,53]. Traditional agronomic measurements and analysis that treat vegetation variables in isolation may fail to capture the full variability in plant and soil function, but the high-resolution, real-time data captured through NIRS in this study offers a promising tool for monitoring changes in soil and plants and their interactions, enabling more adaptive and data-informed land management strategies [54,55]. NIRS can detect subtle changes in forage quality linked to vegetation structure [56]. The use of NIRS technology in remote and proximal sensing improves ecosystem-level nutrient monitoring [20,28]. It has been confirmed in other research that the use of NIRS for real-time assessment of pasture quality under variable management is effective [20]. This aligns with the current research which shows the effective use of high-resolution NIRS in the detection of the interaction effects that traditional sampling methods may overlook, strengthening the interpretation of plant–soil dynamics. The general findings of this study highlight the importance of maintaining both sufficient vegetation cover and appropriate structure or height to improve agricultural landscapes. Cover is essential for building and maintaining soil organic matter and moderating pH, both of which are critical for nutrient availability, microbial health, and long-term productivity [57,58].
Overall, the main findings of this study are well-supported by previous research in grassland ecology, plant physiology, and soil science. The results highlight the key role of vegetation cover in controlling soil processes and show that both plant height and cover together influence plant nutritional quality. These findings are consistent with the current ecosystem theory, which focuses on functional interactions rather than single structural measurements. Height, on the other hand, plays a significant role in determining the nutritional quality of vegetation cover. Managing sward height through controlled grazing, mowing, or rotational practices may help balance forage fibre content with digestibility and energy values [30]. Moreover, the observed interactions in the current study suggest that vegetation cover and height cannot be managed in isolation. For instance, promoting tall vegetation without ensuring sufficient density may reduce forage quality or slow soil OM inputs. Conversely, overly dense low-growing vegetation might enhance soil carbon but offer less nutritional value. Therefore, integrated management approaches that consider how the ground is covered, that is, vegetation cover or density, alongside the vegetation height (adequate species selected for desired structure) are necessary to optimise outcomes in mixed-use agricultural landscapes [23]. Further investigation of the use of vegetation cover and height (density) data to develop a model for the prediction of soil organic matter and pH in farmland is suggested.
5. Conclusions
The current study showed that both vegetation height and cover significantly affect both soil and plant properties in temperate agricultural systems. The interaction between vegetation height and cover significantly affected several plant nutrients: ADF, NDF, DM, DM digestibility, oil, water-soluble carbohydrate, and crude protein. Few effects of vegetation height and cover were found in relation to soil. Higher vegetation cover was associated with increased soil OM stock and reduced soil pH. In land with tall and high vegetation cover, the soil-to-plant OM ratio appears to reach a plateau of about 10:1. The real-time data captured through NIRS offers a promising tool for monitoring changes in soil and plants and their interactions, such as soil OM stock and soil pH, to generate data that can better inform land management practices.
Author Contributions
Conceptualization, S.-O.U.U. and M.J.B.; methodology, S.-O.U.U. and M.J.B.; formal analysis, S.-O.U.U. and M.J.B.; resources, M.J.B.; data curation, S.-O.U.U., W.K.P.N., and M.J.B.; writing—original draft preparation, S.-O.U.U., L.K.W., A.P.W., and M.J.B.; writing—review and editing, S.-O.U.U., L.K.W., A.P.W., W.K.P.N., M.J.B., and T.B.; supervision, L.K.W., A.P.W., and M.J.B.; project administration, S.-O.U.U., L.K.W., A.P.W., M.J.B., and T.B.; funding acquisition, M.J.B. and T.B. All authors have read and agreed to the published version of the manuscript.
Funding
This research study was funded by the Tertiary Education Trust Fund (TETFUND), Nigeria. Soil and plant sample collection was funded by the Farming in Protected Landscapes Programme (created by Defra and delivered locally by the Cotswolds National Landscape team), the Douglas Bomford Trust, and the John Oldacre Trust.
Data Availability Statement
The data that support the findings of this study are available on request from the corresponding author. The study is part of a PhD thesis.
Acknowledgments
We are grateful to all farms included in the study, the support of the Gloucestershire Wildlife Trust, and the help with fieldwork from Greta Jauernik.
Conflicts of Interest
The authors declare no competing interests.
Abbreviations
The following abbreviations are used in this manuscript:
| NIRS | Near-infrared spectroscopy |
| UK | United Kingdom |
| SD | Standard deviation |
| OM | Organic matter |
| N | Total nitrogen |
| DM | Dry matter |
| ADF | Acid detergent fibre |
| NDF | Neutral detergent fibre |
| DMD | Dry matter digestibility |
| FW | Fresh weight |
References
- Udofia, S.O.U.; Williams, L.K.; Wills, A.P.; Bell, M.J. Importance of Vegetation Cover in Organic Systems. In Advances in Organic Farming; CABI: Wallingford, UK, 2025; pp. 163–174. [Google Scholar] [CrossRef] [Scilit]
- Fornara, D.A.; Tilman, D. Plant functional composition influences rates of soil carbon and nitrogen accumulation. J. Ecol. 2008, 96, 314–322. [Google Scholar] [CrossRef] [Scilit]
- Bardgett, R.D.; Van der Putten, W.H. Belowground biodiversity and ecosystem functioning. Nature 2014, 515, 505–511. [Google Scholar] [CrossRef] [Scilit]
- Neina, D. The role of soil pH in plant nutrition and soil biota activity: A review. Soil Syst. 2019, 3, 15. [Google Scholar] [CrossRef] [Scilit]
- Six, J.; Bossuyt, H.; Degryze, S.; Denef, K. A history of research on the link between (micro) aggregates, soil biota, and soil organic matter dynamics. Soil Till. Res. 2004, 79, 7–31. [Google Scholar] [CrossRef] [Scilit]
- Gentsch, N.; Riechers, F.L.; Boy, J.; Schweneker, D.; Feuerstein, U.; Heuermann, D.; Guggenberger, G. Cover crops improve soil structure and change organic carbon distribution in macroaggregate fractions. Soil 2024, 10, 139–155. [Google Scholar] [CrossRef] [Scilit]
- Lisec, T.; Šibanc, N.; Lojen, S.; Vidrih, T. Sustainable grassland management systems affect soil physicochemical properties and forage nutritional quality. Plants 2024, 13, 838. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tilman, D.; Reich, P.B.; Knops, J.M.H. Biodiversity and ecosystem stability in a decade long grassland experiment. Nature 2001, 441, 629–632. [Google Scholar] [CrossRef] [Scilit]
- Crosse, S.; O’Donovan, M.; Delaby, L.; Boland, T.M. Quantifying the effect of sward characteristics on the nutritive value of grass herbage. Grass Forage Sci. 2015, 70, 364–377. [Google Scholar] [CrossRef] [Scilit]
- Bell, M.J.; Mereu, L.; Davis, J. The use of mobile near-infrared spectroscopy for real-time pasture management. Front. Sustain. Food Syst. 2018, 2, 76. [Google Scholar] [CrossRef] [Scilit]
- Reinermann, S.; Rathmann, J.; Lüker Jans, N.; Schmidtlein, S. Grassland yield estimations—Potentials and limitations of remote sensing. Biogeosciences 2025, 22, 4969–4983. [Google Scholar] [CrossRef] [Scilit]
- Franzluebbers, A.J. Soil organic matter stratification ratio as an indicator of soil quality. Soil Till. Res. 2002, 66, 95–106. [Google Scholar] [CrossRef] [Scilit]
- Hobbs, R.J.; Higgs, E.; Harris, J.A. Novel ecosystems: Implications for conservation and restoration. Trends Ecol. Evol. 2008, 24, 599–605. [Google Scholar] [CrossRef] [Scilit]
- UK Centre for Ecology & Hydrology (UKCEH). Less Intensively Managed Grasslands Have Higher Plant Diversity and Better Soil Health. UKCEH Website. 2022. Available online: https://www.ceh.ac.uk/press/less-intensively-managed-grasslands-have-higher-plant-diversity-and-better-soil-health (accessed on 18 October 2025).
- Jerrentrup, J.S.; Wrage Mönnig, N.; Röver, K.U.; Isselstein, J. Grazing with different livestock species affects the plant and insect diversity of species-rich grasslands. Agric. Ecosyst. Environ. 2020, 287, 106679. [Google Scholar] [CrossRef] [Scilit]
- Gibon, A. Managing grassland for production, the environment and the landscape. Livest. Prod. Sci. 2005, 96, 11–31. [Google Scholar] [CrossRef] [Scilit]
- Batello, C.; Mannetje, L.; Martinez, A.; Suttie, J. Plant Genetic Resources of Forage Crops, Pasture and Rangelands. Thematic Background Study; FAO Report. 2008, pp. 5–7. Available online: https://www.fao.org/fileadmin/templates/agphome/documents/PGR/SoW2/thematicstudy_forage.pdf (accessed on 15 October 2025).
- Wilkins, P.W.; Humphreys, M.O. Progress in breeding perennial forage grasses for temperate agriculture. J. Agric. Sci. 2003, 140, 129–150. [Google Scholar] [CrossRef] [Scilit]
- Wrage, N.; Strodthoff, J.; Cuchillo, H.M.; Isselstein, J.; Kayser, M. Phytodiversity of temperate permanent grasslands: Ecosystem services for agriculture and livestock management for diversity conservation. Biodivers. Conserv. 2011, 20, 3317–3339. [Google Scholar] [CrossRef] [Scilit]
- Bell, M.J.; Huggett, Z.J.; Slinger, K.R.; Roos, F. Effect of pasture cover and height on nutrient concentrations in diverse swards in the UK. Grassl Sci. 2021, 67, 267–272. [Google Scholar] [CrossRef] [Scilit]
- Poorter, H.; Niklas, K.J.; Reich, P.B.; Oleksyn, J.; Poot, P.; Mommer, L. Biomass allocation to leaves, stems and roots: Meta-analyses of interspecific variation and environmental control. New Phytol. 2012, 193, 30–50. [Google Scholar] [CrossRef] [Scilit]
- Lemaire, G.; Gastal, F.; Franzluebbers, A.; Chabbi, A. Grassland–cropping rotations: An avenue for agricultural diversification to reconcile high production with environmental quality. J. Environ. Manag. 2015, 56, 1065–1077. [Google Scholar] [CrossRef] [Scilit]
- Wilson, J.R.; Hatfield, R.D. Structural and chemical changes of cell wall types during stem development: Consequences for fibre degradation by rumen microflora. Aust. J. Agric. Res. 1997, 48, 165–180. [Google Scholar] [CrossRef] [Scilit]
- Buxton, D.R. Quality-related characteristics of forages as influenced by plant environment and agronomic factors. Anim. Feed Sci. Technol. 1996, 59, 37–49. [Google Scholar] [CrossRef] [Scilit]
- Buxton, D.R.; Redfearn, D.D. Plant limitations to fiber digestion and utilization. J. Nutr. 1997, 127, 814S–818S. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Valencia Gómez, E.; Galland, T.; Carmona, C.; Goberna, M.; Götzenberger, L.; Lepš, J.; Verdú, M.; Macek, P.; Bello, F.D. The functional structure of plant communities drives soil functioning via changes in soil abiotic properties. Ecology 2022, 103, e3833. [Google Scholar] [CrossRef] [Scilit]
- Coleman, S.W.; Moore, J.E.; Wilson, J.R. Quality and utilization. Warm-Seas. (C4) Grasses 2004, 45, 267–308. [Google Scholar] [CrossRef] [Scilit]
- Mainetti, A.; Ravetto Enri, S.; Pittarello, M.; Lombardi, G.; Lonati, M. Main ecological and environmental factors affecting forage yield and quality in Alpine summer pastures (NW-Italy, Gran Paradiso National Park). Grass Forage Sci. 2023, 78, 254–267. [Google Scholar] [CrossRef] [Scilit]
- Peìrez-Harguindeguy, N.; Díaz, S.; Garnier, E.; Lavorel, S.; Poorter, H.; Jaureguiberry, P.; Bret-Harte, M.S.; Cornwell, W.K.; Joseph Craine, J.; Gurvich, D.E.; et al. New handbook for standardised measurement of plant functional traits worldwide. Aust. J. Bot. 2013, 61, 167–234. [Google Scholar] [CrossRef] [Scilit]
- Li, T.; Zhang, X.; Zou, M.; Chen, J.; Hou, F. Grazing management of cultivated grassland with different weed propor-tions optimizes soil nutrient status and improves forage yield and nutritional quality. Field Crops Res. 2025, 331, 110018. [Google Scholar] [CrossRef] [Scilit]
- Jobbágy, E.G.; Jackson, R.B. The vertical distribution of soil organic carbon and its relation to climate and vegetation. Ecol. Appl. 2000, 10, 423–436. [Google Scholar] [CrossRef]
- Lal, R. Soil carbon sequestration to mitigate climate change. Geoderma 2004, 123, 1–22. [Google Scholar] [CrossRef] [Scilit]
- Wardle, D.A.; Bardgett, R.D.; Klironomos, J.N.; Setala, H.; Van Der Putten, W.H.; Wall, D.H. Ecological linkages between aboveground and belowground biota. Science 2004, 304, 1629–1633. [Google Scholar] [CrossRef] [Scilit]
- Yang, Y.; Gunina, A.; Cheng, H.; Liu, L.; Wang, B.; Dou, Y.; Wang, Y.; Liang, C.; An, S.; Chang, S.X. Unlocking mechanisms for soil organic matter accumulation: Carbon use efficiency and microbial necromass as the keys. Glob. Change Biol. 2025, 31, e70033. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Conant, R.T.; Paustian, K.; Elliott, E.T. Grassland management and conversion into grassland: Effects on soil carbon. Ecol. Appl. 2001, 11, 343–355. [Google Scholar] [CrossRef]
- Six, J.; Conant, R.T.; Paul, E.A.; Paustian, K. Stabilization mechanisms of soil organic matter: Implications for C-saturation of soils. Plant Soil. 2002, 241, 155–176. [Google Scholar] [CrossRef] [Scilit]
- Post, W.M.; Kwon, K.C. Soil carbon sequestration and land-use change: Processes and potential. Glob. Change Biol. 2000, 6, 317–327. [Google Scholar] [CrossRef] [Scilit]
- You, X.; Li, S.; Zhang, T.; Wang, Y. Vegetation structure regulates soil nutrient dynamics in grassland ecosystems under changing climates. J. Appl. Ecol. 2024, 61, 45–59. [Google Scholar] [CrossRef] [Scilit]
- Lal, R. Soil carbon sequestration impacts on global climate change and food security. Science 2004, 304, 1623–1627. [Google Scholar] [CrossRef] [Scilit]
- Rousk, J.; Bååth, E.; Brookes, P.C.; Lauber, C.L.; Lozupone, C.; Caporaso, J.G.; Knight, R.; Fierer, N. Soil bacterial and fungal communities across a pH gradient in an arable soil. ISME J. 2010, 4, 1340–1351. [Google Scholar] [CrossRef] [Scilit]
- Ritchie, G.S.P.; Dolling, P.J. The role of organic matter in soil acidification. Aust. J. Soil Res. 1985, 23, 569–576. [Google Scholar] [CrossRef] [Scilit]
- Haynes, R.J.; Swift, R.S. Effects of soil acidification and subsequent leaching on levels of extractable nutrients in a soil. Plant Soil 1986, 95, 327–336. [Google Scholar] [CrossRef] [Scilit]
- Tiemann, L.K.; Grandy, A.S.; Atkinson, E.E.; Marin-Spiotta, E.; McDaniel, M.D. Crop rotational diversity enhances belowground communities and functions in an agroecosystem. Ecol. Lett. 2015, 18, 761–771. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- De Deyn, G.B.; Van der Putten, W.H. Linking aboveground and belowground diversity. Trends Ecol. Evol. 2005, 20, 625–633. [Google Scholar] [CrossRef] [Scilit]
- Levy, P.; Bentley, L.; Danks, P.; Emmett, B.; Garbutt, A.; Heming, S.; Henrys, P.; Keith, A.; Lebron, I.; McNamara, N.; et al. The effects of land use on soil carbon stocks in the UK. Biogeosciences 2024, 21, 4301–4315. [Google Scholar] [CrossRef] [Scilit]
- Abanda, P.A.; Compton, J.S.; Hannigan, R.E. Soil nutrient content, above-ground biomass and litter in a semi-arid shrubland, South Africa. Geoderma 2011, 164, 128–137. [Google Scholar] [CrossRef] [Scilit]
- Allart, L.; Joly, F.; Oostvogels, V.; Mosnier, C.; Gross, N.; Ripoll-Bosch, R.; Dumont, B. Farmers’ perceptions of permanent grasslands and their intentions to adapt to climate change influence their resilience strategy. Renew. Agric. Food Syst. 2024, 39, e33. [Google Scholar] [CrossRef] [Scilit]
- Zamora, C.G. Impacts of Reduced Tillage and Disturbance on Soil Health and Microbial Community Dynamics in Grass Seed Cropping Systems. 2023. Available online: https://ir.library.oregonstate.edu/concern/graduate_thesis_or_dissertations/j6731b990 (accessed on 12 October 2025).
- Buxton, D.R.; Marten, G.C. Forage quality of plant parts of perennial grasses and relationship to phenology. Crop Sci. 1989, 29, 429–435. [Google Scholar] [CrossRef] [Scilit]
- da Silveira Pontes, L.; Giostri, A.F.; Baldissera, T.C.; Barro, R.S.; Stafin, G.; Porfírio-da-Silva, V.; Moletta, J.L.; César de Faccio Carvalho, P. Interactive effects of trees and nitrogen supply on the agronomic characteristics of warm-climate grasses. Agron. J. 2016, 108, 1531–1541. [Google Scholar] [CrossRef] [Scilit]
- Whitehead, D.C. Nutrient Elements in Grassland: Soil–Plant Animal Relationships; CABI: Wallingford, UK, 2000. [Google Scholar]
- Babiker, E.E.; El Sheikh, E.A.; Osman, A.J.; El Tinay, A.H. Effect of nitrogen fixation, nitrogen fertilization and viral infection on yield, tannin and protein contents and in vitro protein digestibility of faba bean. Plant Food Hum. Nutr. 1995, 47, 257–263. [Google Scholar] [CrossRef] [Scilit]
- Schmitz, O.J.; Buchkowski, R.W.; Burghardt, K.T.; Donihue, C.M. Functional traits and trait-mediated interactions: Connecting community-level interactions with ecosystem functioning. In Advances in Ecological Research; Academic Press: Cambridge, MA, USA, 2015; Volume 52, pp. 319–343. [Google Scholar] [CrossRef] [Scilit]
- Brown, D.J.; Shepherd, K.D.; Walsh, M.G.; Mays, M.D.; Reinsch, T.G. Global soil characterization with VNIR diffuse re-flectance spectroscopy. Geoderma 2018, 132, 273–290. [Google Scholar] [CrossRef] [Scilit]
- Stuth, J.; Jama, A.; Tolleson, D. Direct and indirect means of predicting forage quality through near infrared reflectance spectroscopy. Field Crops Res. 2003, 84, 45–56. [Google Scholar] [CrossRef] [Scilit]
- Julitta, T. Optical Proximal Sensing for Vegetation Monitoring. 2015. Available online: https://tesidottorato.depositolegale.it/handle/20.500.14242/170988 (accessed on 10 October 2025).
- Vitousek, P.M.; Menge, D.N.L.; Reed, S.C.; Cleveland, C.C. Biological nitrogen fixation: Rates, patterns and ecological controls in terrestrial ecosystems. Philos. Trans. R. Soc. B Biol. Sci. 2010, 365, 1215–1225. [Google Scholar] [CrossRef] [Scilit]
- Bashir, O.; Ali, T.; Baba, Z.A.; Rather, G.H.; Bangroo, S.A.; Mukhtar, S.D.; Naik, N.; Mohiuddin, R.; Bharati, V.; Bhat, R.A. Soil organic matter and its impact on soil properties and nutrient status. In Microbiota and Biofertilizers, Vol 2: Ecofriendly Tools for Reclamation of Degraded Soil Environs; Springer International Publishing: Cham, Switzerland, 2021; pp. 129–159. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.