


Abstract
Seed imbibition and germination under water stress conditions are critical determinants of successful crop establishment; therefore, understanding imbibition responses under osmotic stress is essential for improving seed quality assessment and management strategies for crop production under suboptimal water availability. This study aimed to analyze the effect of reduced water potential on the imbibition curve and triphasic pattern of seeds in several Solanaceae species. The study used seeds from three Solanaceae crops—chili (Capsicum annuum L., varieties Simpatik and Sempurna), tomato (Solanum lycopersicum L., varieties Niki and Rempai), and eggplant (Solanum melongena L., varieties Tangguh and Provita). The seeds were subjected to various levels of osmotic stress using polyethylene glycol (PEG 6000) to simulate water potentials of 0.00, −0.30, −1.90, and −4.10 MPa. Lower water potential in the growing medium reduced the seed’s ability to absorb the water. The triphasic pattern consistently appeared only in chili seeds, whereas in tomatoes and eggplants, it varied across varieties and water potential conditions. Lower water potential delayed the end of Phase I and prolonged the duration of Phase II. These findings confirm that the standard imbibition pattern cannot be generalized to all seeds, and therefore, the imbibition response is specific to seed type, variety, and germination environment.
1. Introduction
Seed germination marks a pivotal transition in the plant life cycle, linking a quiescent, desiccated seed to an actively growing seedling capable of independent establishment. Germination success depends largely on environmental factors, particularly water availability [1]. Water not only initiates the physical swelling of the seed but also triggers a cascade of metabolic and physiological processes necessary for embryo activation and growth [2,3]. The initial uptake of water, known as imbibition, is fundamental to germination because it rehydrates cellular components and restores membrane integrity, and triggers metabolic processes essential for embryo activation and subsequent seedling development [4,5,6]. However, when the surrounding medium exhibits reduced water potential, such as under drought or osmotic stress, the rate and extent of imbibition are adversely affected, potentially delaying, reducing, or completely inhibiting germination [7,8].
According to [3], the process of seed imbibition follows a triphasic pattern. In the first phase (Phase I), water absorption occurs rapidly due to potential differences between the seed and the germination medium, and by low-intensity metabolic activity. The second phase (Phase II) is characterized by a plateau in water absorption, where the seed reaches near-hydration equilibrium. However, there is little to no change and intense metabolic activities involved in preparing the seed for germination and seedling growth. Next, the third phase (Phase III) is characterized by subsequent growth with radicle protrusion and seed weight gain, all of which are sensitive to water availability. Reduced water potential slows or blocks the imbibition process and thereby delays the germination process [9]. In particular, prolongation of phase II under low water potential correlates with delayed radicle emergence and slower progression toward germination completion [1], while the same hydric constraint aligns with observations of slowed imbibition and germination under drought or osmotic stress across multiple species [2]. These findings collectively establish water potential as a primary modulator of the imbibition timeline and germination rate [2].
The Solanaceae family includes agriculturally important crops (Capsicum and Solanum species) that are frequently cultivated under water-limited conditions, making them relevant for studying seed germination in drought-like environments [10,11]. Seed germination under drought-like environments is a critical stage determining stand establishment and yield, making it a pertinent focal point for understanding drought tolerance in solanaceous crops [12,13].
This contextualizes them, making them ideal models for studying the influence of water potential on imbibition and the triphasic pattern. Previous studies have reported that Solanaceae seeds are sensitive to reduced water potential, showing delayed radicle emergence and decreased final germination percentage as osmotic stress intensifies [14,15,16]. Furthermore, analyzing the imbibition curve under reduced water potential provides valuable information for modeling seed hydration kinetics. Parameters derived from these curves, such as the rate of water absorption and the duration of each imbibition phase, can be used to describe species-specific differences and to identify thresholds of water limitation that impede germination. Therefore, the present study aims to evaluate the effect of reduced water potential on the imbibition curve and the triphasic pattern of seeds in selected Solanaceae species. The hypothesis of this research is that reduced water potential significantly affects the seed imbibition curve and the triphasic imbibition pattern in Solanaceae species.
2. Materials and Methods
This research was conducted at the Seed Physiology and Health Laboratory, Department of Agronomy and Horticulture, Faculty of Agriculture, Bogor Agricultural University, from April to September 2025. The main materials used in this research include seeds from three commodities of the Solanaceae family, namely chilies (Simpatik and Sempurna varieties), tomatoes (Niki and Rempai varieties), and eggplants (Tangguh and Provita varieties). The selection of varieties was conducted to represent differences in fruit morphology (size, shape, type, and color), where Rempai has small round fruits and Niki has large elongated fruits; Simpatik is a large red chili, while Sempurna is a red curly chili; and Tangguh produces purple fruits, whereas Provita produces green, round fruits. The experiment was conducted separately for each variety and was arranged in a randomized complete block design (RCBD) with a single factor, namely osmotic potential, comprising four levels [0.0 MPa (control), −0.30, −1.90, and −4.10 MPa] induced by different concentrations of polyethylene glycol 6000 (PEG 6000) solutions. Each treatment was replicated four times, resulting in a total of 16 experimental units (4 levels × 4 replications). Each experimental unit within the block consisted of 72 plastic boxes, with each box containing 50 seeds. These 72 boxes were further divided into two groups: 36 boxes for moisture content determination and 36 boxes for radicle emergence observation. Both variables were observed over four-hour intervals, starting from 0 h until no more radicles emerged. The concentrations of PEG 6000 required to obtain these values were determined by using the following equation [17], Ψ = [−0.10 − 0.001C + 0.026C2 − 0.0003C3], where Ψ is the osmotic potential (MPa) and C is the concentration (g L−1 PEG 6000 in water). As the control, a solution with osmotic potential Ψ = 0.0 MPa was used.
The research procedure began with germination of 50 seeds in each germination on a double layer of paper and towel tissue soaked in at least 10 mL of the PEG 6000 solution in a tightly sealed plastic box (17 cm × 11.5 cm × 7.5 cm). The boxes were stored in a germination room with a temperature ranging from 25 °C ± 2 °C. Water content and radicle emergence observations were carried out for four-hour intervals, from 0 h until no more radicles emerged. Radicle emergence was defined as the seed emergence of a radicle reaching 2 mm in length. Both parameters used a new seed sample for each imbibition event. Radicle emergence (RE) was calculated using the following formula:
Seed moisture content was measured using the direct method using a high-temperature oven at 130 °C for 1 h, with each testing unit consisting of 50 seeds. The measurement results are expressed as a percentage of water content absorbed by the seeds, using the following formula [18]:
Water content patterns for each commodity and water potential during imbibition were analyzed using a regression model in Minitab 18. The equation model used is as follows:
where a, b, c, and d are constants; x is the imbibition time; and y is the seed water content (%).
y = a + bx + cx2 + dx3
The regression model was used to determine the classic imbibition curve proposed by [19], which contains three phases: phase 1: fast imbibition; phase 2: little to no imbibition, usually longer than phase 1; and phase 3: radicle protrusion and water content increases again. Phase I, Phase II (lag phase), and Phase III were identified based on the extreme points of the first derivative of the third-degree polynomial equation. The first derivative represents the rate of change (hydration rate), and phase transitions were determined by solving the condition y′ = 0. The resulting real roots indicate the change points, i.e., the time points at which the rate of water uptake changes direction. Model validity was evaluated using ANOVA, demonstrating that the regression models were statistically significant (p < 0.05) and there was agreement between the fitted curves and observed water content values within their respective standard deviations for each treatment.
Radicle emergence (RE) was recorded at regular time intervals. A seed was considered germinated when the radicle protruded at least 2 mm. Final radicle emergence (final RE, %) was calculated as the percentage of germinated seeds at the end of the observation period. Time to First RE was defined as the time (hours) at which the first radicle protrusion was observed in each replicate. The time required to reach 50% emergence (T50) was calculated using the formula
where N is the final number of emerged seeds, and ni and nj are the cumulative seed emergence at times ti and tj.
Data were analyzed using one-way ANOVA, and mean comparisons were performed using Duncan’s Multiple Range Test (DMRT) at the 5% significance level.
3. Results
3.1. Seed Water Content
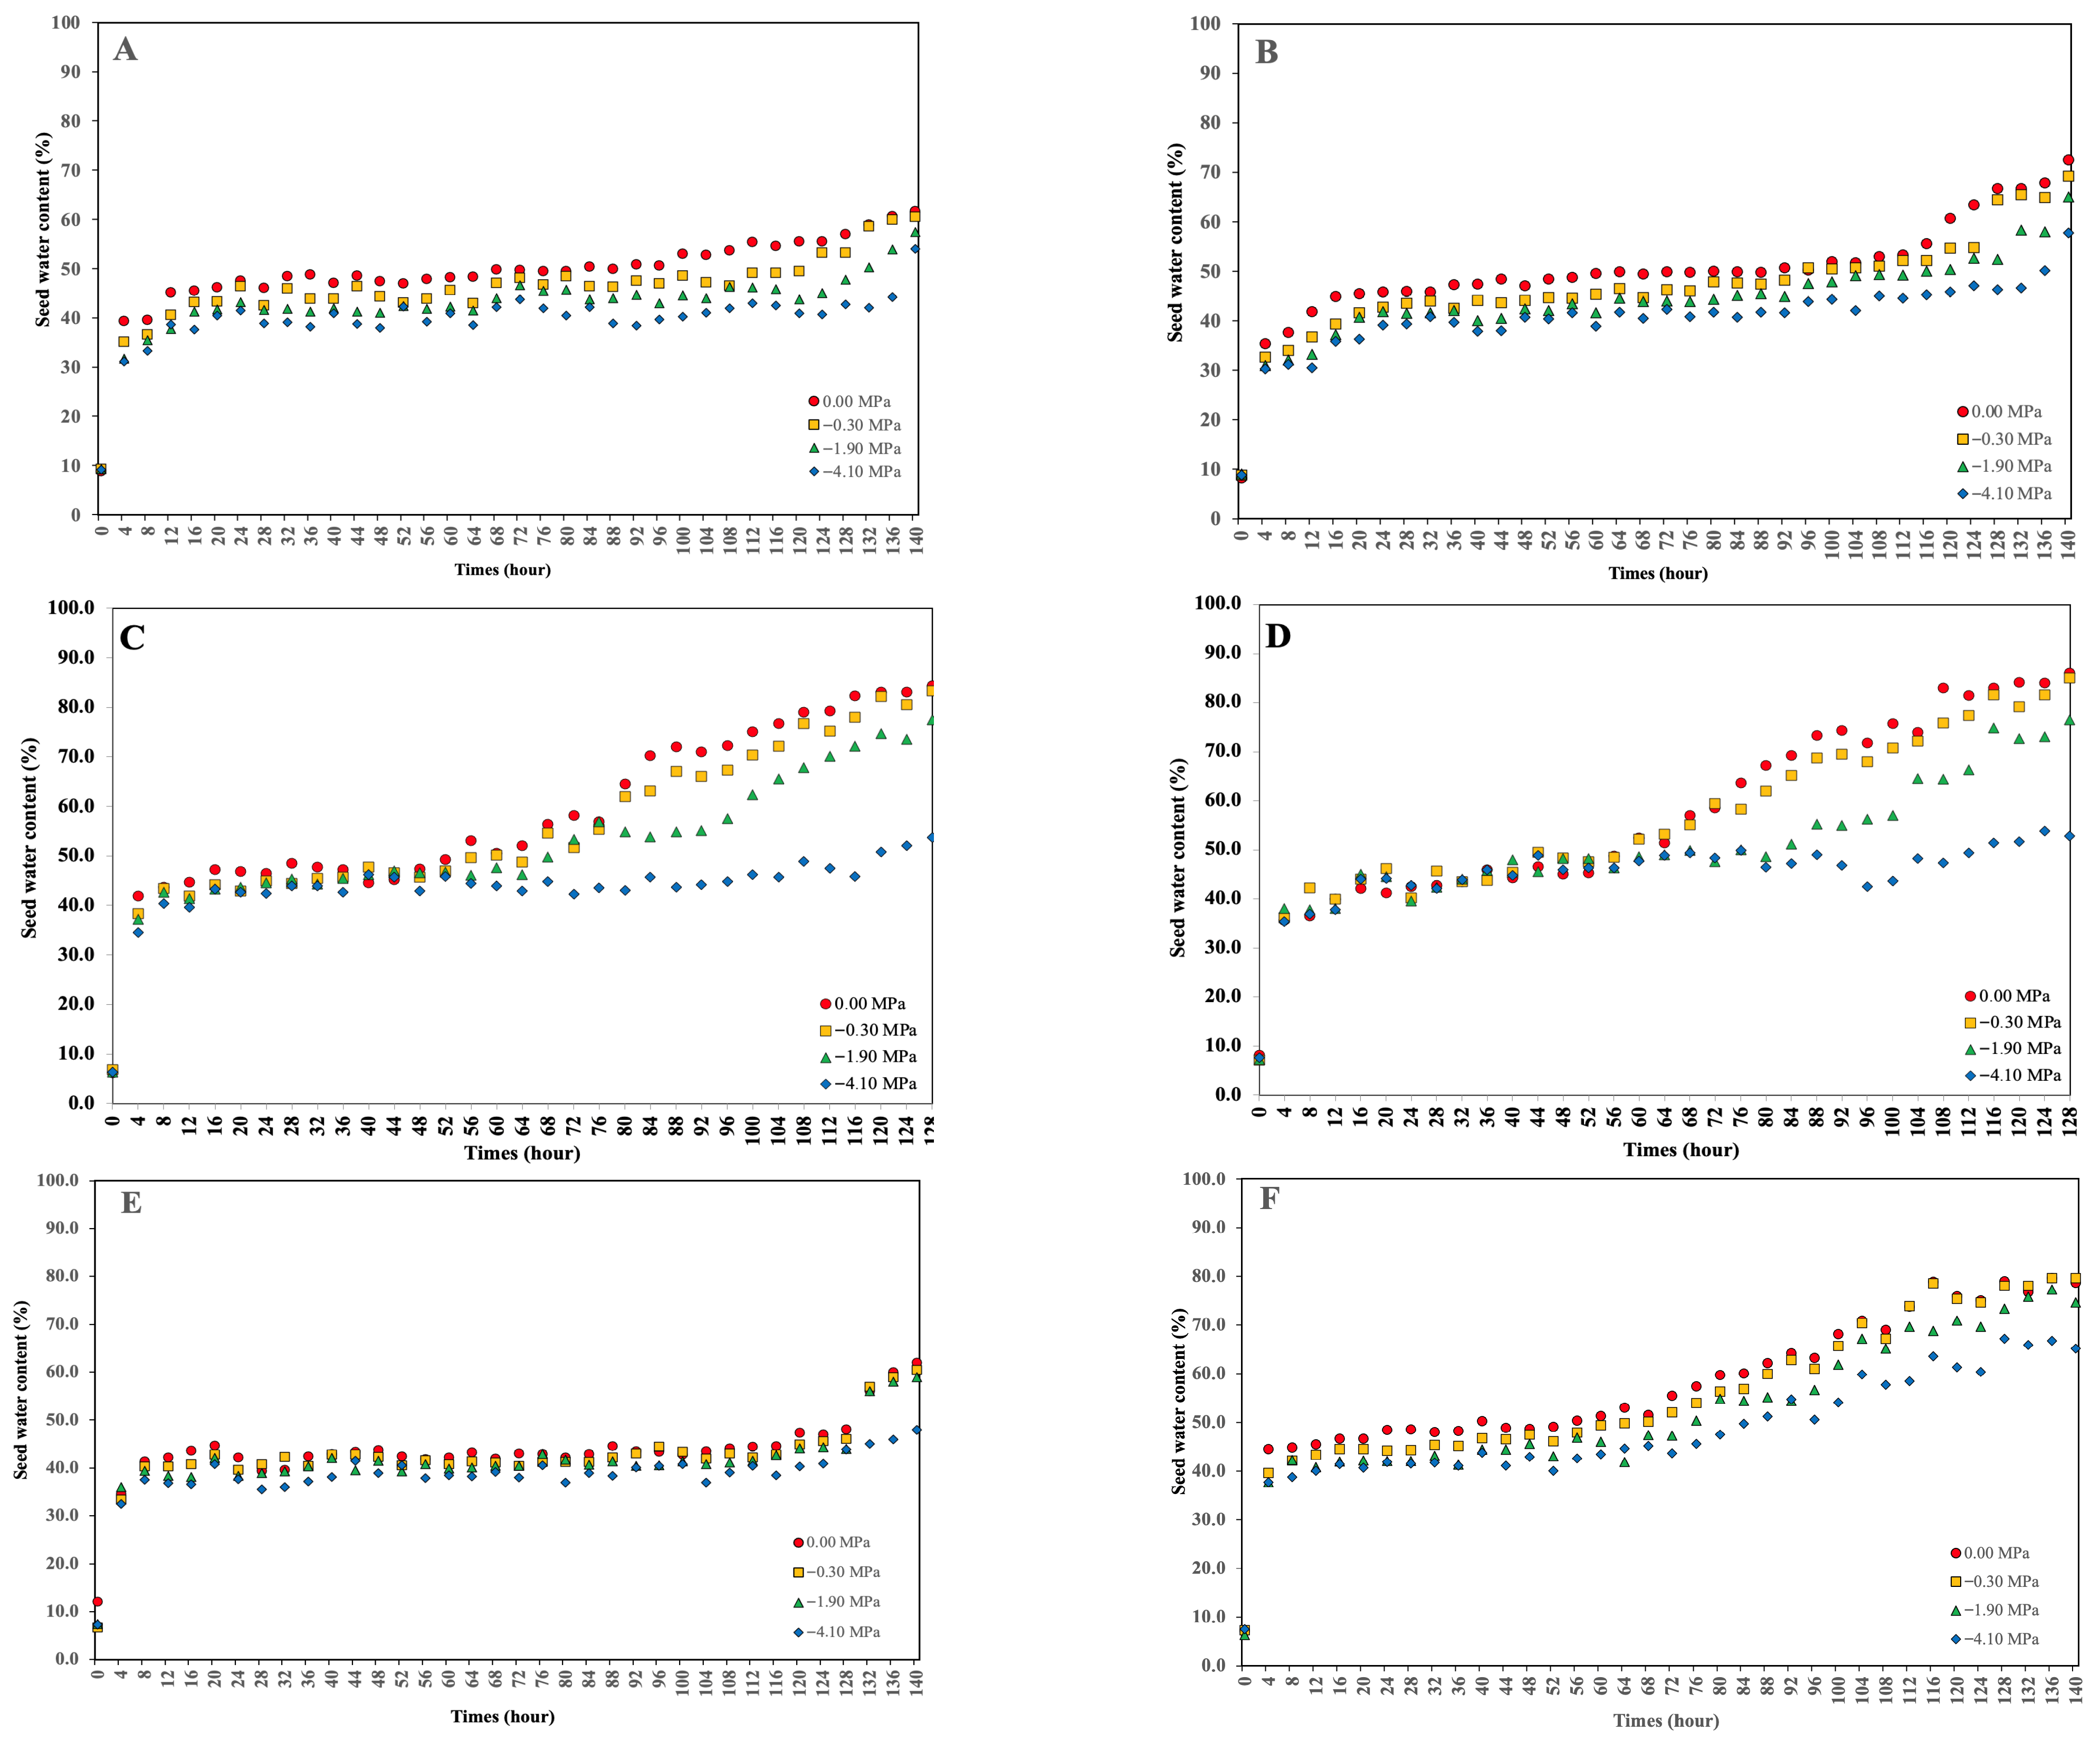
The results show that seed water content increases with imbibition time at each water potential. Lower water potential (more negative) reduces the rate of water uptake by seeds (Figure 1). Figure 1A,B show that the water content at 140 h for 0.00 MPa is 61.6% and 72.5%, respectively, for the Simpatik and Sempurna varieties. Compared with −4.1 MPa, the water content at the same time shows differences of 7.6% and 14.7%. Tomato seeds of the Niki and Rempai varieties (Figure 1C,D) tend to have higher water content. At the end of the observation, the water content of the Niki and Rempai varieties at 0.00 MPa reached 84.3% and 86.1%, respectively, and, compared with −4.10 MPa at the same time, showed differences of 33.3% and 30.6%. Figure 1E,F on eggplant seeds of the Tangguh and Provita varieties show that the water content at the end of the observation for 0 MPa is 62.0% and 78.7%, respectively. Compared with −4.10 MPa, the water content at the same time shows differences of 14.0% and 13.5%.
Figure 1.
Seed water content pattern of chili seed varieties Simpatik (A) and Sempurna (B); tomato seed varieties Niki (C) and Rempai (D); and eggplant seed varieties Tangguh (E) and Provita (F) on four water potential levels.
The pattern and rate of water uptake vary with environmental conditions, particularly the surrounding water potential, which determines the driving force for water movement into the seed. Under osmotic stress, the rate of imbibition typically decreases, delaying subsequent physiological events. The data presented in Figure 1 serve as the basis for establishing the mathematical relationship between seed water content and imbibition time across different water potentials. The third-degree polynomial regression equations for each commodity are presented in Table 1.
Table 1.
Third-degree polynomial regression equations describing the relationship between seed water content (y) and imbibition time (x) of chili, tomato, and eggplant seeds under different water potential levels.
For chili seed, the regression models show a strong fit, with coefficients of determination (R2) ranging from 66.69% to 79.08% for the Simpatik variety and 84.19% to 90.21% for the Sampurna variety. For tomato seed, R2 ranged from 69.31% to 89.10% for the Niki variety and from 76.31% to 92.81% for the Rempai variety. Moreover, for eggplant seed, R2 ranged from 53.13% to 89.10% for the Tangguh variety and 82.48% to 88.03% for the Provita variety. The results show that the third-degree polynomial function effectively describes the relationship between time and water content. The intercept and slope coefficients vary according to water potential, reflecting the influence of osmotic stress on the rate and extent of seed water absorption. In general, the highest R2 values were observed at 0.0 MPa and −0.30 MPa, suggesting that the model fits the data better under non-stress or mild-stress conditions. The gradual decrease in regression coefficients at lower water potentials (−1.90 MPa and −4.10 MPa) indicates reduced water uptake efficiency and a slower imbibition rate as osmotic pressure increased. Among the two varieties for each commodity, the higher R2 Sempurna, Rempai, and Provita varieties imply more consistent water absorption behavior under varying water potentials. In Table 1, the p-value indicates whether each third-degree polynomial regression model significantly describes the relationship between imbibition time and seed water content at a given water potential. Treatments with p < 0.05 (mostly <0.01) show that the polynomial terms significantly explain changes in water content over time, meaning the triphasic imbibition pattern is statistically supported. This is evident in most chili and eggplant treatments, where the third-degree polynomial structure reliably captures hydration dynamics. However, several tomato and eggplant (e.g., Provita) treatments show p > 0.05, despite relatively high R2 values.
3.2. Seed Imbibition Pattern and Radicle Emergence
3.2.1. Chili Seed
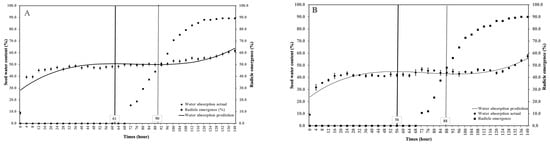
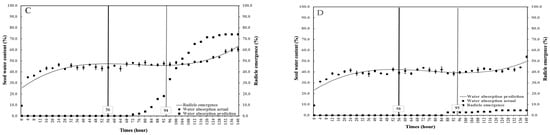
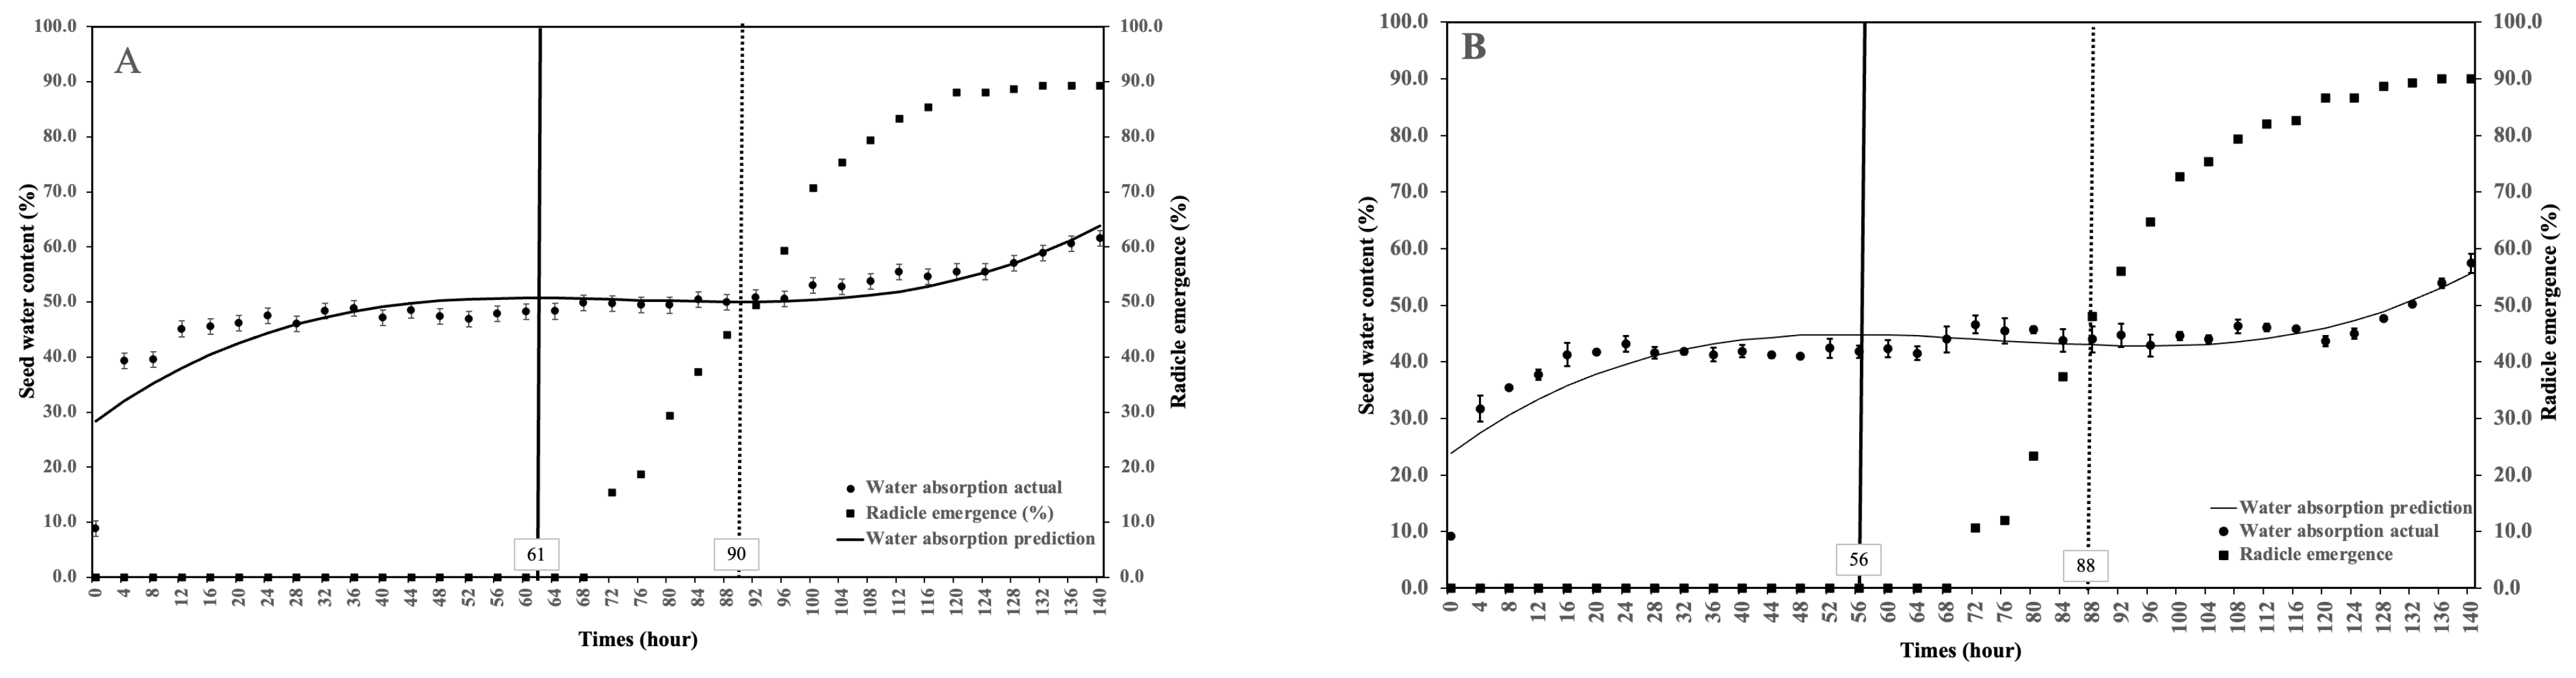
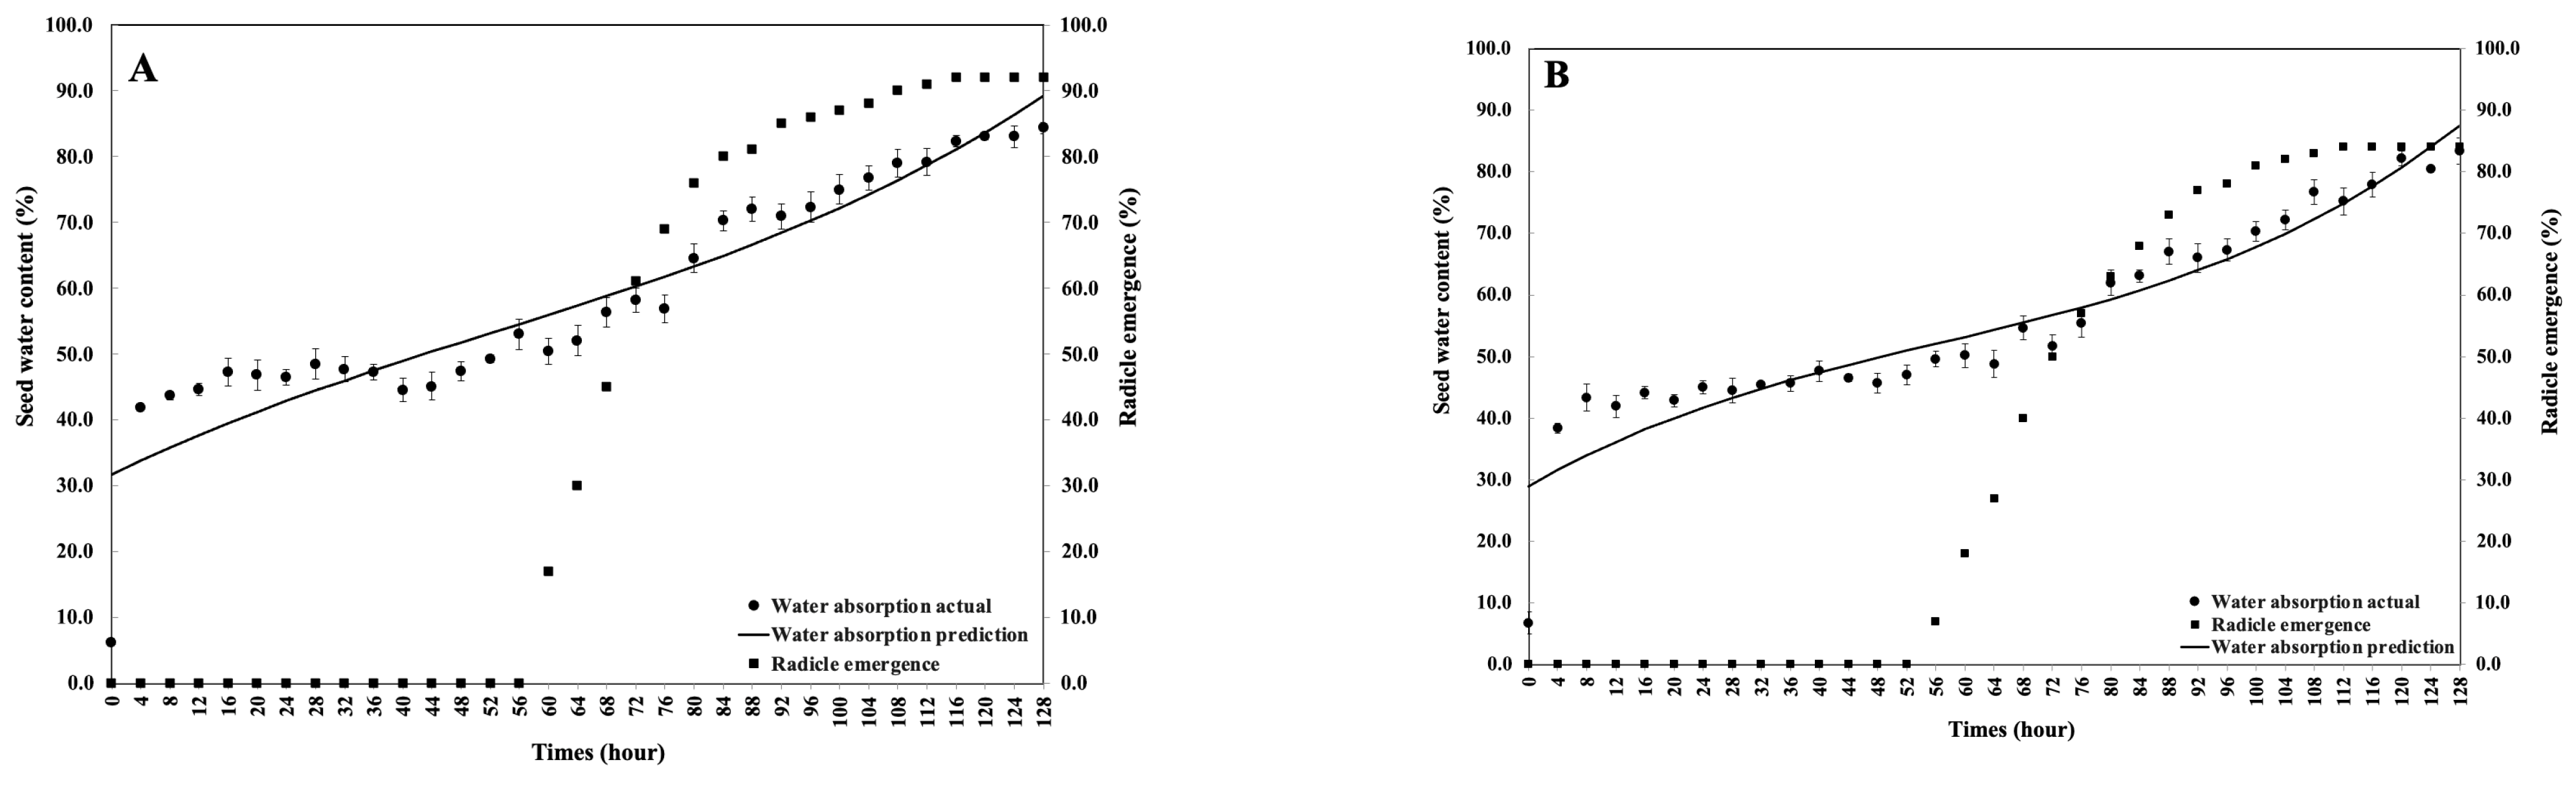
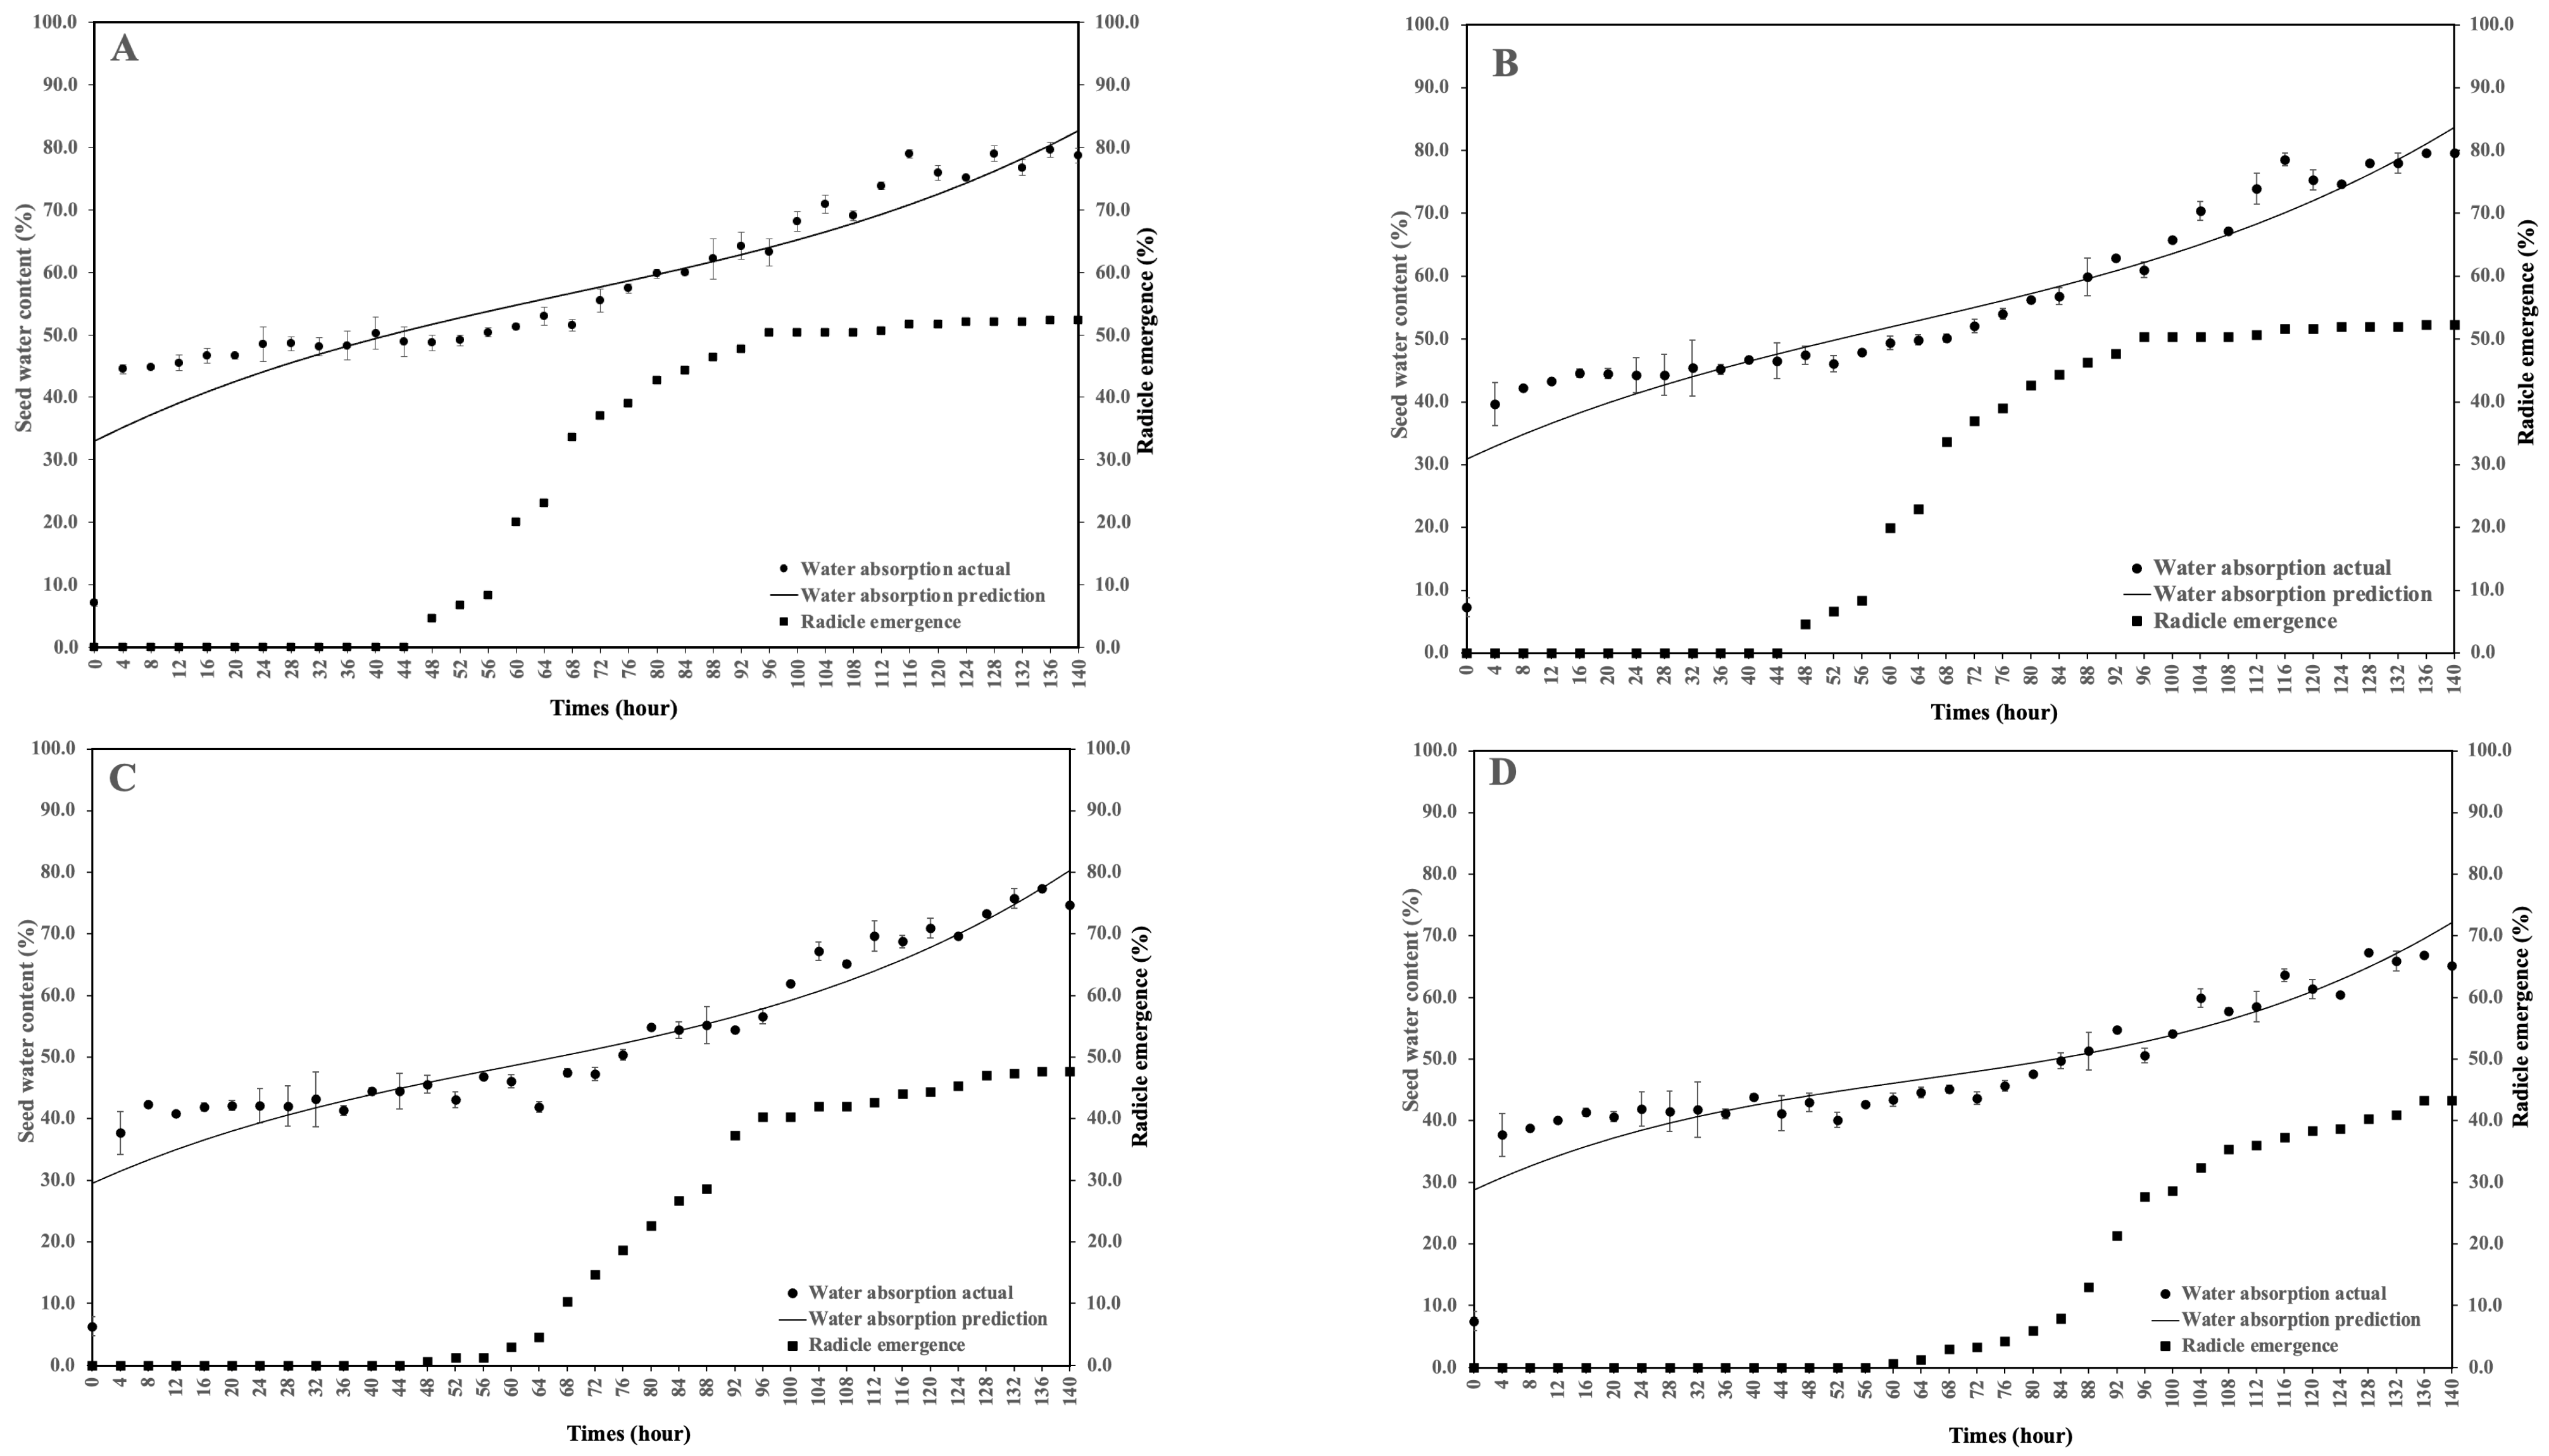
The typical triphasic imbibition pattern was observed in both Simpatik (Figure 2A–D) and Sempurna (Figure 3A–D) varieties. In the Simpatik variety (Figure 2), Phase I lasted ~56–60 h across treatments, while decreasing water potential progressively prolonged Phase II and delayed the onset of Phase III—from ~88–90 h in Figure 2A,B to ~94–95 h in Figure 2C,D—resulting in reduced radicle emergence, particularly under −4.1 MPa (Figure 2D). A similar trend was observed in the Sempurna variety (Figure 3), where Phase I remained relatively stable (~52–58 h; Figure 3A–C), but Phase II lengthened as water potential decreased, delaying Phase III onset to ~94 h under −4.1 MPa (Figure 3D) and markedly suppressing radicle emergence. Overall, as shown in Figure 2 and Figure 3, reduced water potential primarily extended the lag phase and delayed seedling establishment in both varieties. In the Simpatik variety (Figure 3), radicle emergence (RE) began during the mid-to-late portion of Phase II rather than strictly at the end of Phase II, as classically described in the triphasic model. Theoretical models of seed imbibition generally define Phase III as beginning at the onset of radicle protrusion, implying that RE marks the transition from Phase II to Phase III. However, in the present results, initial RE was observed before the complete transition to Phase III (as indicated by the second change-point of the hydration curve).
Figure 2.
Imbibition and radicle emergence (RE) curves of Simpatik variety of chili seeds at a water potential of 0.0 MPa (A), −0.30 MPa (B), −1.90 MPa (C), and −4.1 MPa (D). Full vertical lines indicate the transition between imbibition phases 1 and 2, and dotted lines indicate the beginning of phase 3.
Figure 3.
Imbibition and radicle emergence curves of Sempurna variety of chili seeds at a water potential of 0.0 MPa (A), −0.30 MPa (B), −1.90 MPa (C), and −4.1 MPa (D). Full vertical lines indicate the transition between imbibition phases 1 and 2 and dotted lines indicate the beginning of phase 3.
Table 2 and Table 3 show that decreasing water potential significantly influenced final radicle emergence (RE), Time to First RE, and T50 (DMRT 5%) in both varieties. In Simpatik (Table 2), final radicle emergence (RE) remained high at 0.00 and −0.30 MPa but declined markedly at −1.90 MPa and was severely reduced at −4.10 MPa, indicating strong inhibition under severe osmotic stress. Time to First RE was stable (72 h) under mild and moderate stress but was significantly delayed at −4.10 MPa (88 h), suggesting slower initiation of visible germination under severe water deficit. T50 increased at −1.90 MPa, reflecting slower germination rate and reduced synchrony, while severe stress further limited germination progression due to the very low final emergence. In Sempurna (Table 3), final RE progressively decreased as water potential became more negative, with substantial reduction at −1.90 MPa and minimal emergence at −4.10 MPa. Time to First RE ranged between 80 and 84 h, showing slight but significant variation under different stress levels, indicating moderate sensitivity during germination initiation. T50 values were significantly affected by water potential, with prolonged germination time under certain stress conditions, reflecting slower metabolic progression and reduced emergence uniformity.
Table 2.
Effects of water potential on final radicle emergence (RE), Time to First RE, and T50 in seeds of the chili variety Simpatik.
Table 3.
Effects of water potential on final radicle emergence (RE), Time to First RE, and T50 in seeds of the chili variety Sempurna.
3.2.2. Tomato Seed
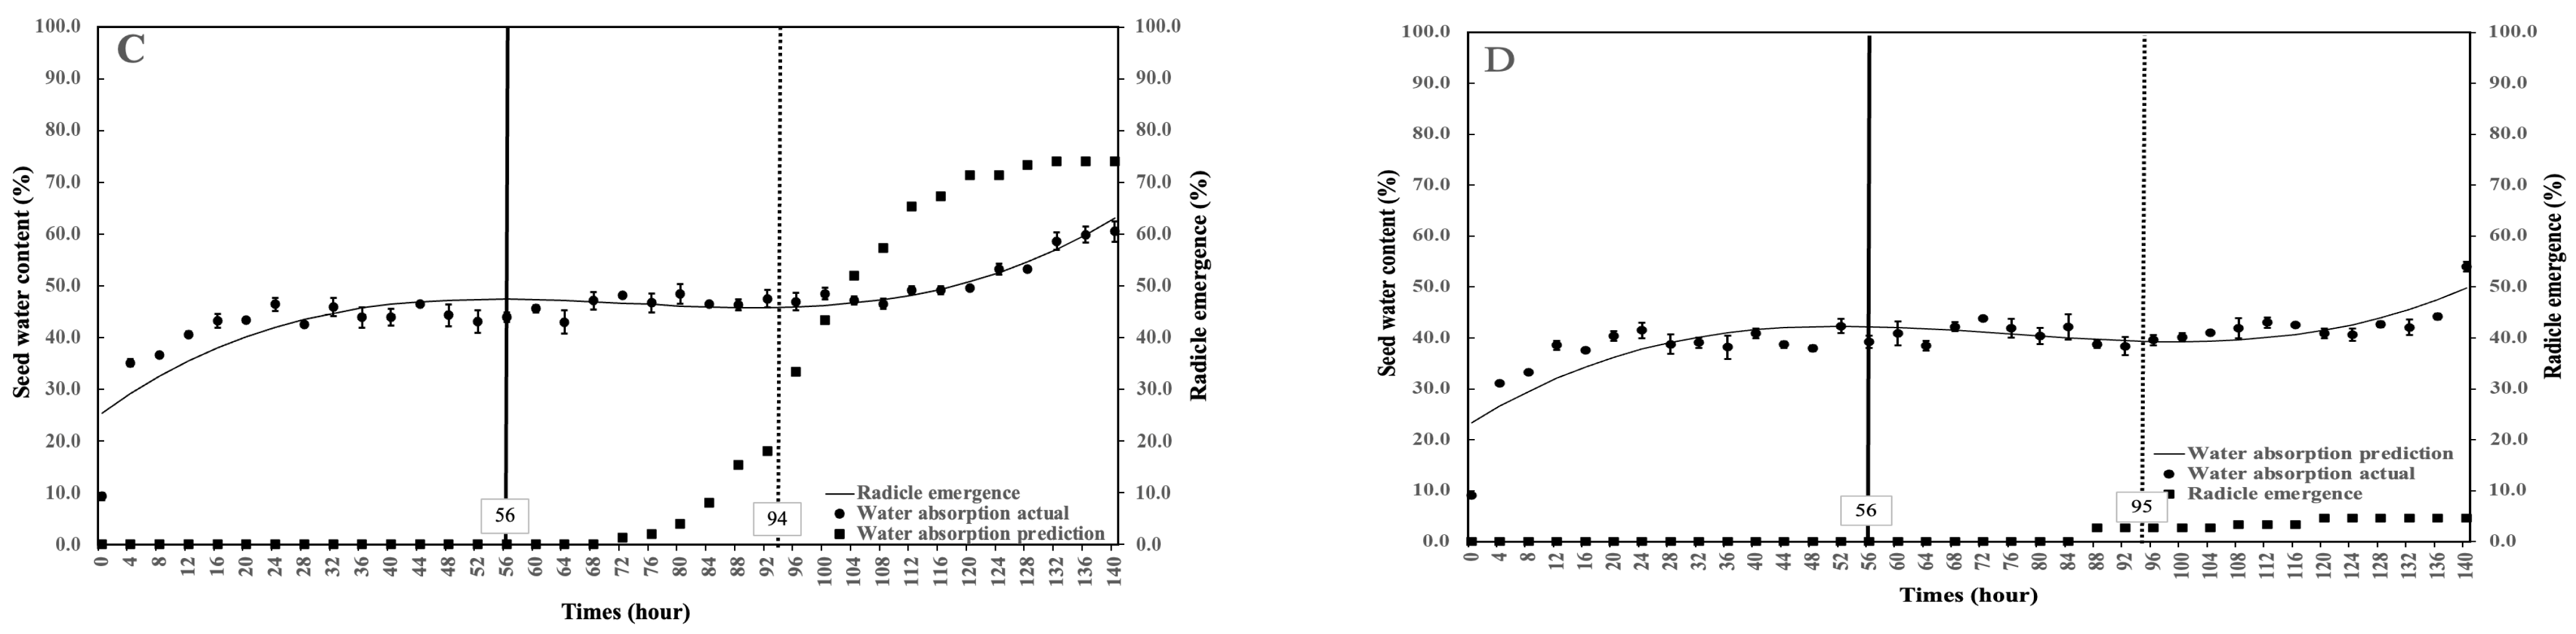
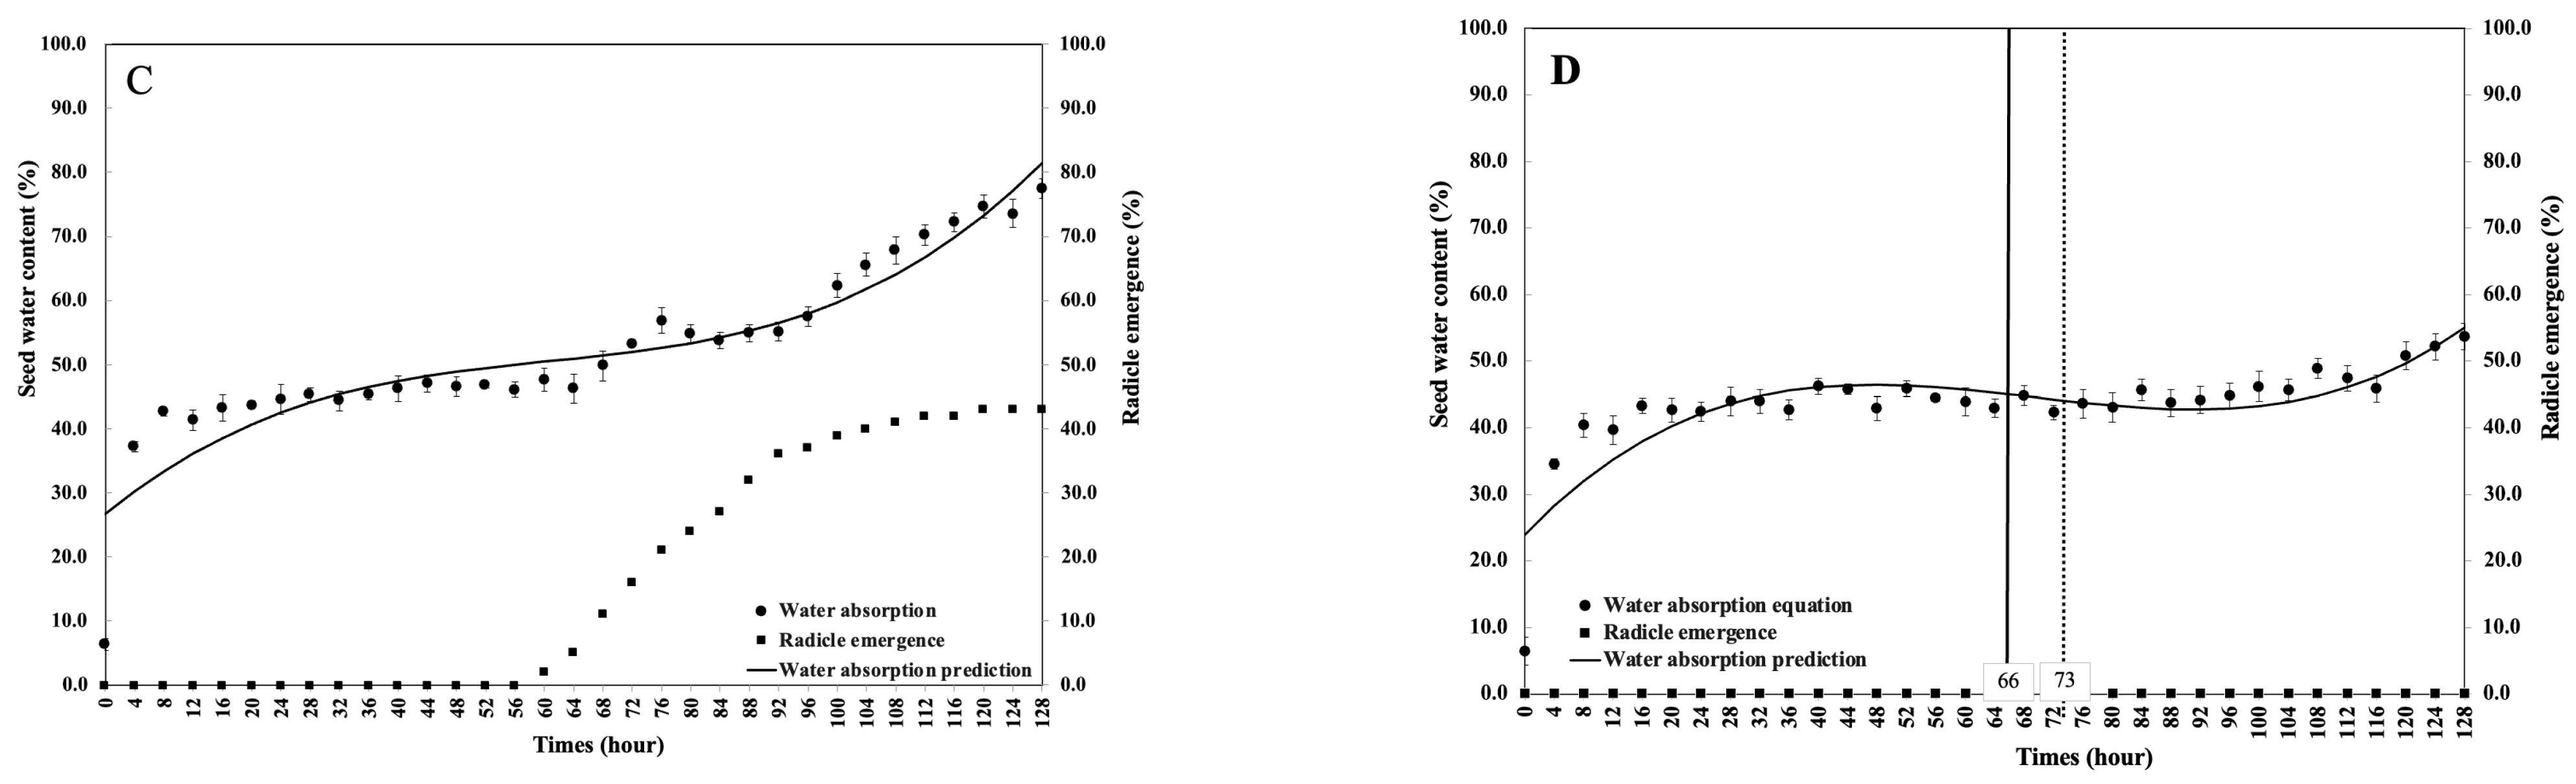
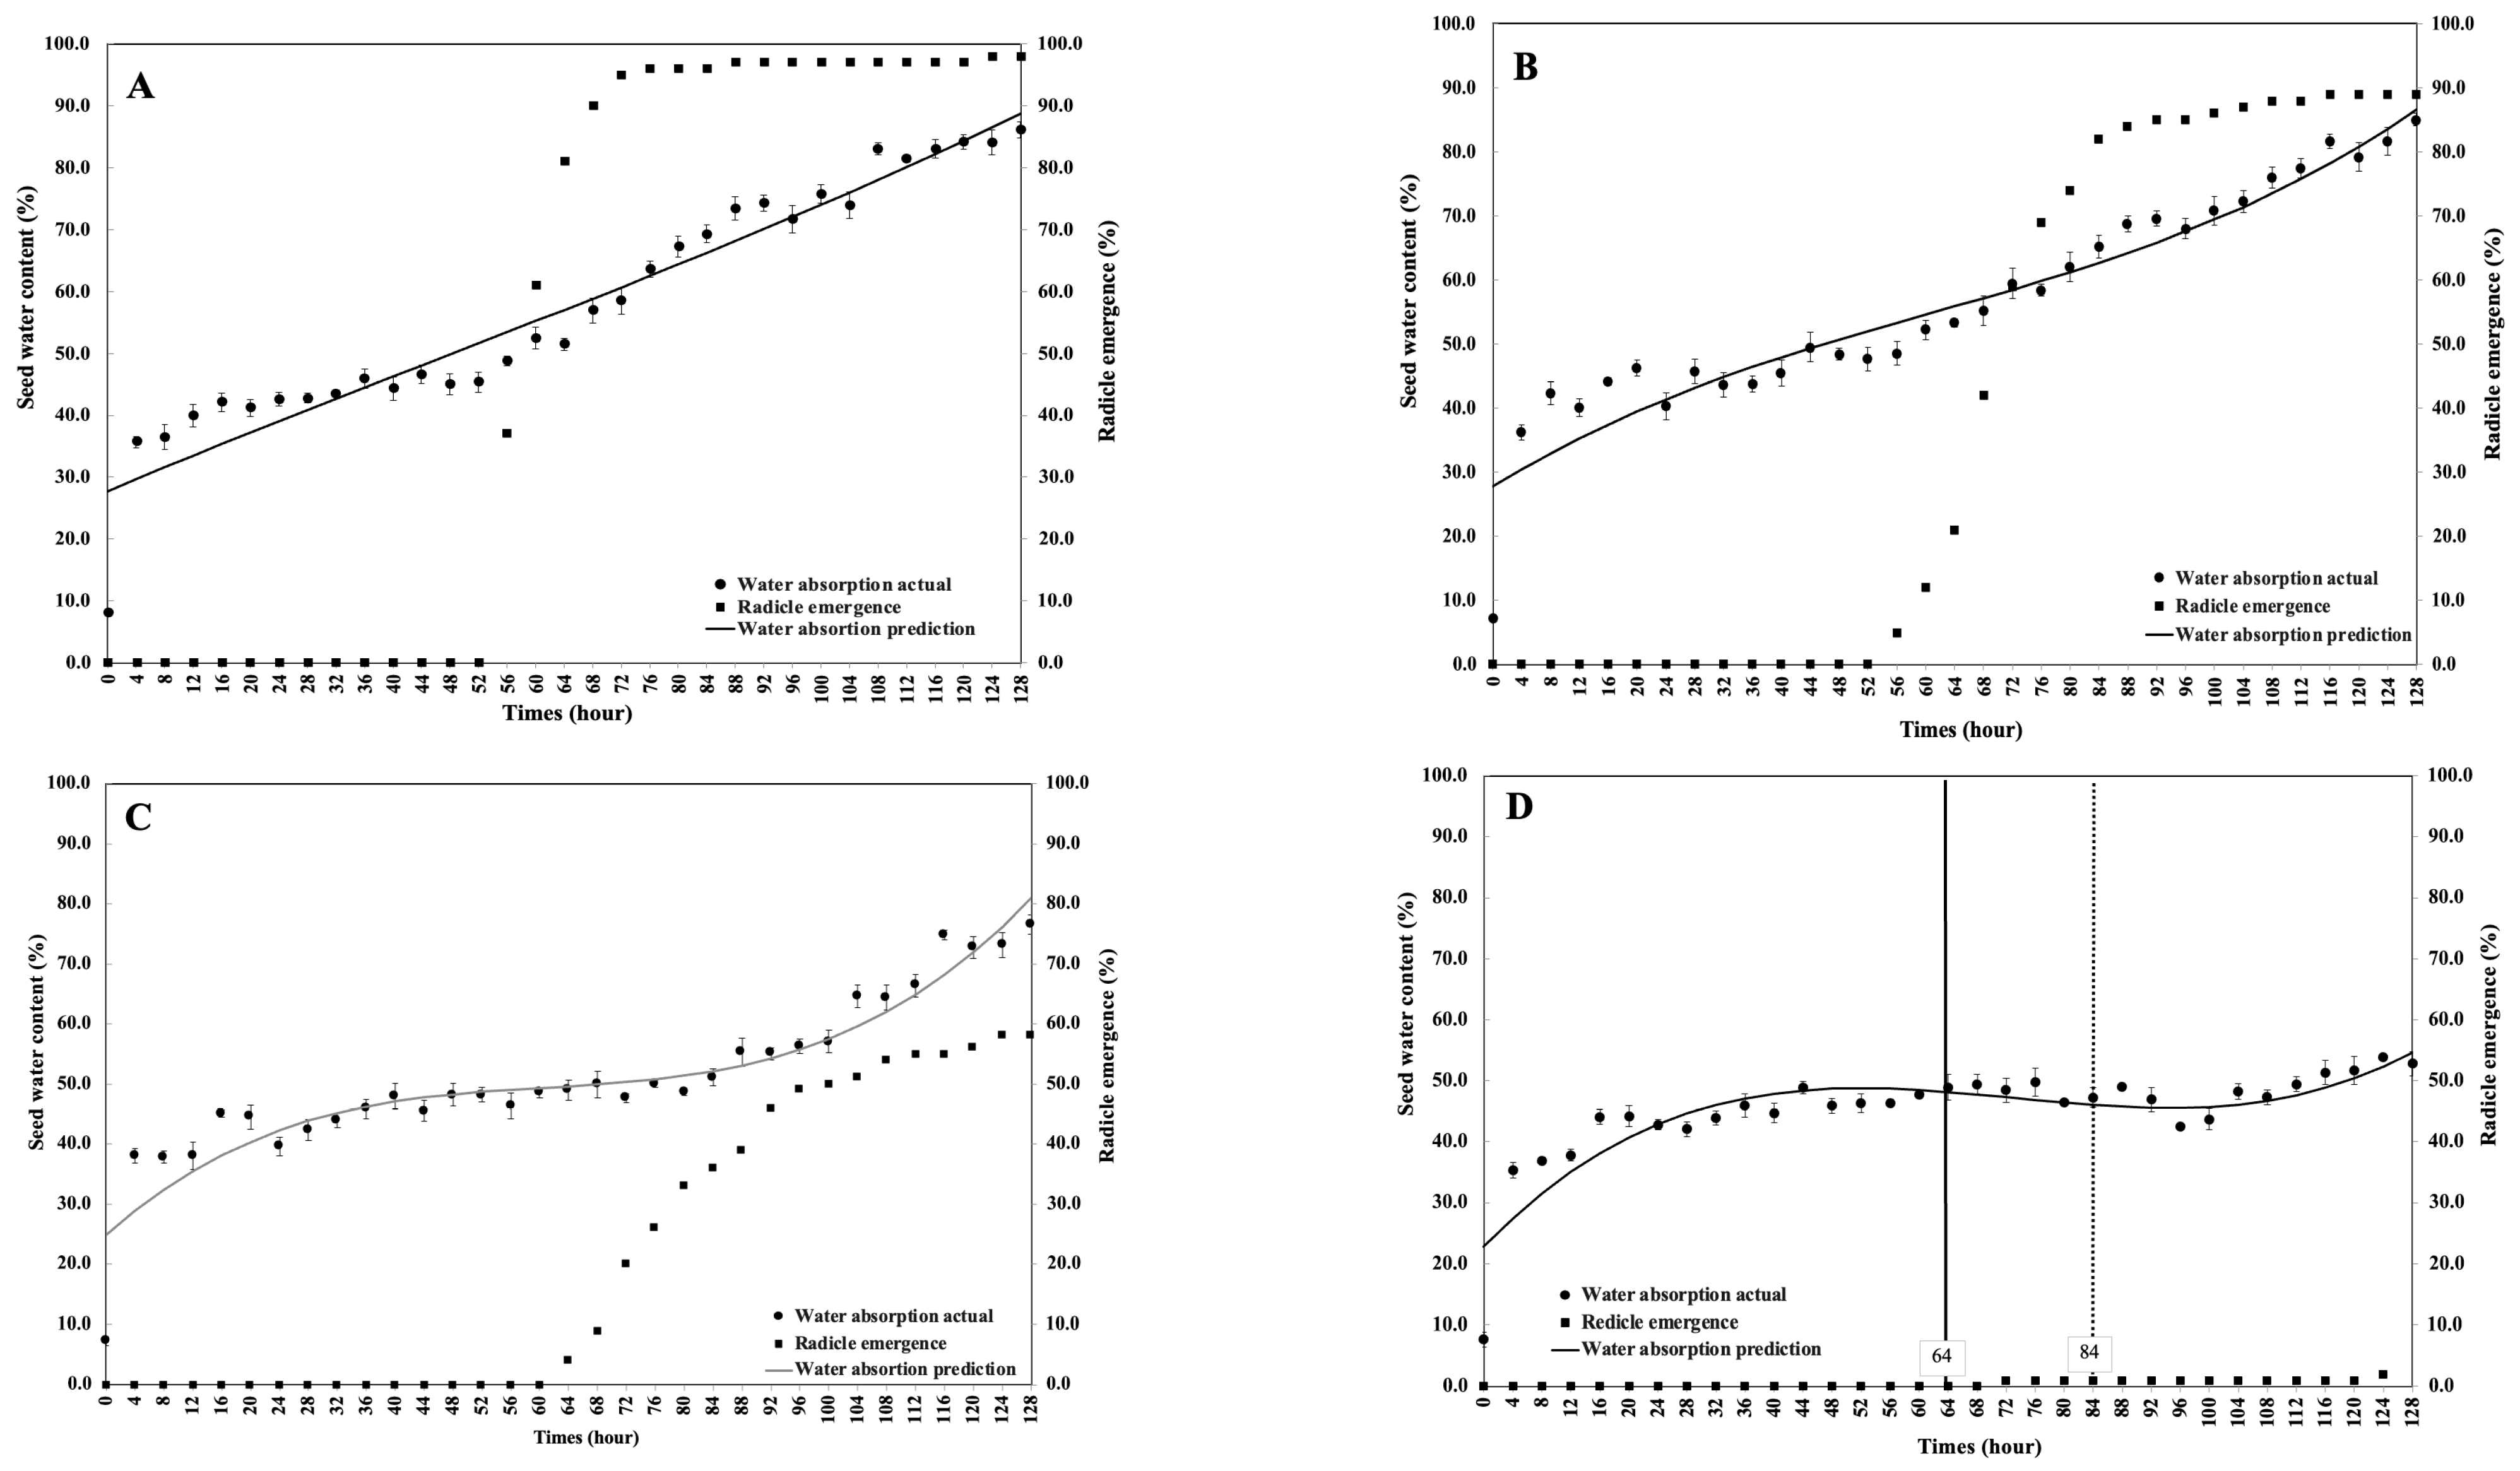
The standard triphasic imbibition pattern was not observed at any water potential level in either tomato seed variety. The triphasic pattern was only identified at −4.10 MPa for the Niki variety (Figure 4) and Rempai variety (Figure 5). At a water potential of −4.10 MPa, the Niki variety reached the end of phases I and II at 66 and 73 h, respectively. However, no germination occurred, because the seeds experienced excessive stress (Figure 4D). At other water potential levels, although the triphasic pattern was not observed, Niki tomato seeds were relatively resistant to −0.30 MPa and −1.90 MPa, as evidenced by radicle emergence rates of 84% and 42%, respectively. Figure 5D shows that in the Rempai variety, the end of phases I and II occurred at 64 and 84 h, respectively. The RE did not appear in the −4.1 MPa treatment because the seeds experienced severe stress.
Figure 4.
Imbibition and radicle emergence curves of Niki variety of tomato seeds at a water potential of 0.0 MPa (A), −0.30 MPa (B), −1.90 MPa (C), and −4.1 MPa (D). Full vertical lines indicate the transition between imbibition phases 1 and 2 and dotted lines indicate the beginning of phase 3.
Figure 5.
Imbibition and radicle emergence curves of Rempai variety of tomato seeds at water potentials of 0.0 MPa (A), −0.30 MPa (B), −1.90 MPa (C), and −4.1 MPa (D). Full vertical lines indicate the transition between imbibition phases 1 and 2 and dotted lines indicate the beginning of phase 3.
Decreasing water potential significantly affected germination performance (DMRT 5%), radicle emergence (RE), Time to First RE, and T50 (DMRT 5%) in Niki and Rempai varieties. In the Niki variety (Table 4), final RE declined progressively from 92.0% at 0.00 MPa to 84.0% at −0.30 MPa and 42.0% at −1.90 MPa, with complete inhibition at −4.10 MPa. Time to First RE remained stable at 56 h under optimal and mild stress but was delayed to 60 h at −1.90 MPa, indicating slower germination initiation under moderate osmotic stress. T50 increased significantly as water potential decreased (from 64 h at 0.00 MPa to 76 h at −1.90 MPa), reflecting reduced germination speed and synchrony under water deficit. No T50 value was observed at −4.10 MPa, due to the absence of emergence. In the Rempai variety (Table 5), the final RE declined progressively from 98.0% at 0.00 MPa to 58.0% at −1.90 MPa and was almost completely inhibited at −4.10 MPa (2.0%), indicating high sensitivity to severe osmotic stress. Time to First RE increased from 56 h under optimal and mild stress to 64 h at −1.90 MPa and 72 h at −4.10 MPa, demonstrating delayed germination initiation under reduced water availability. T50 also increased under moderate stress (78 h at −1.90 MPa), reflecting slower and less synchronized germination, while severe stress drastically limited emergence capacity.
Table 4.
Effects of water potential on final radicle emergence (RE), Time to First RE, and T50 in seeds of the tomato variety Niki.
Table 5.
Effects of water potential on final radicle emergence (RE), Time to First RE, and T50 in seeds of the tomato variety Rempai.
3.2.3. Eggplant Seed
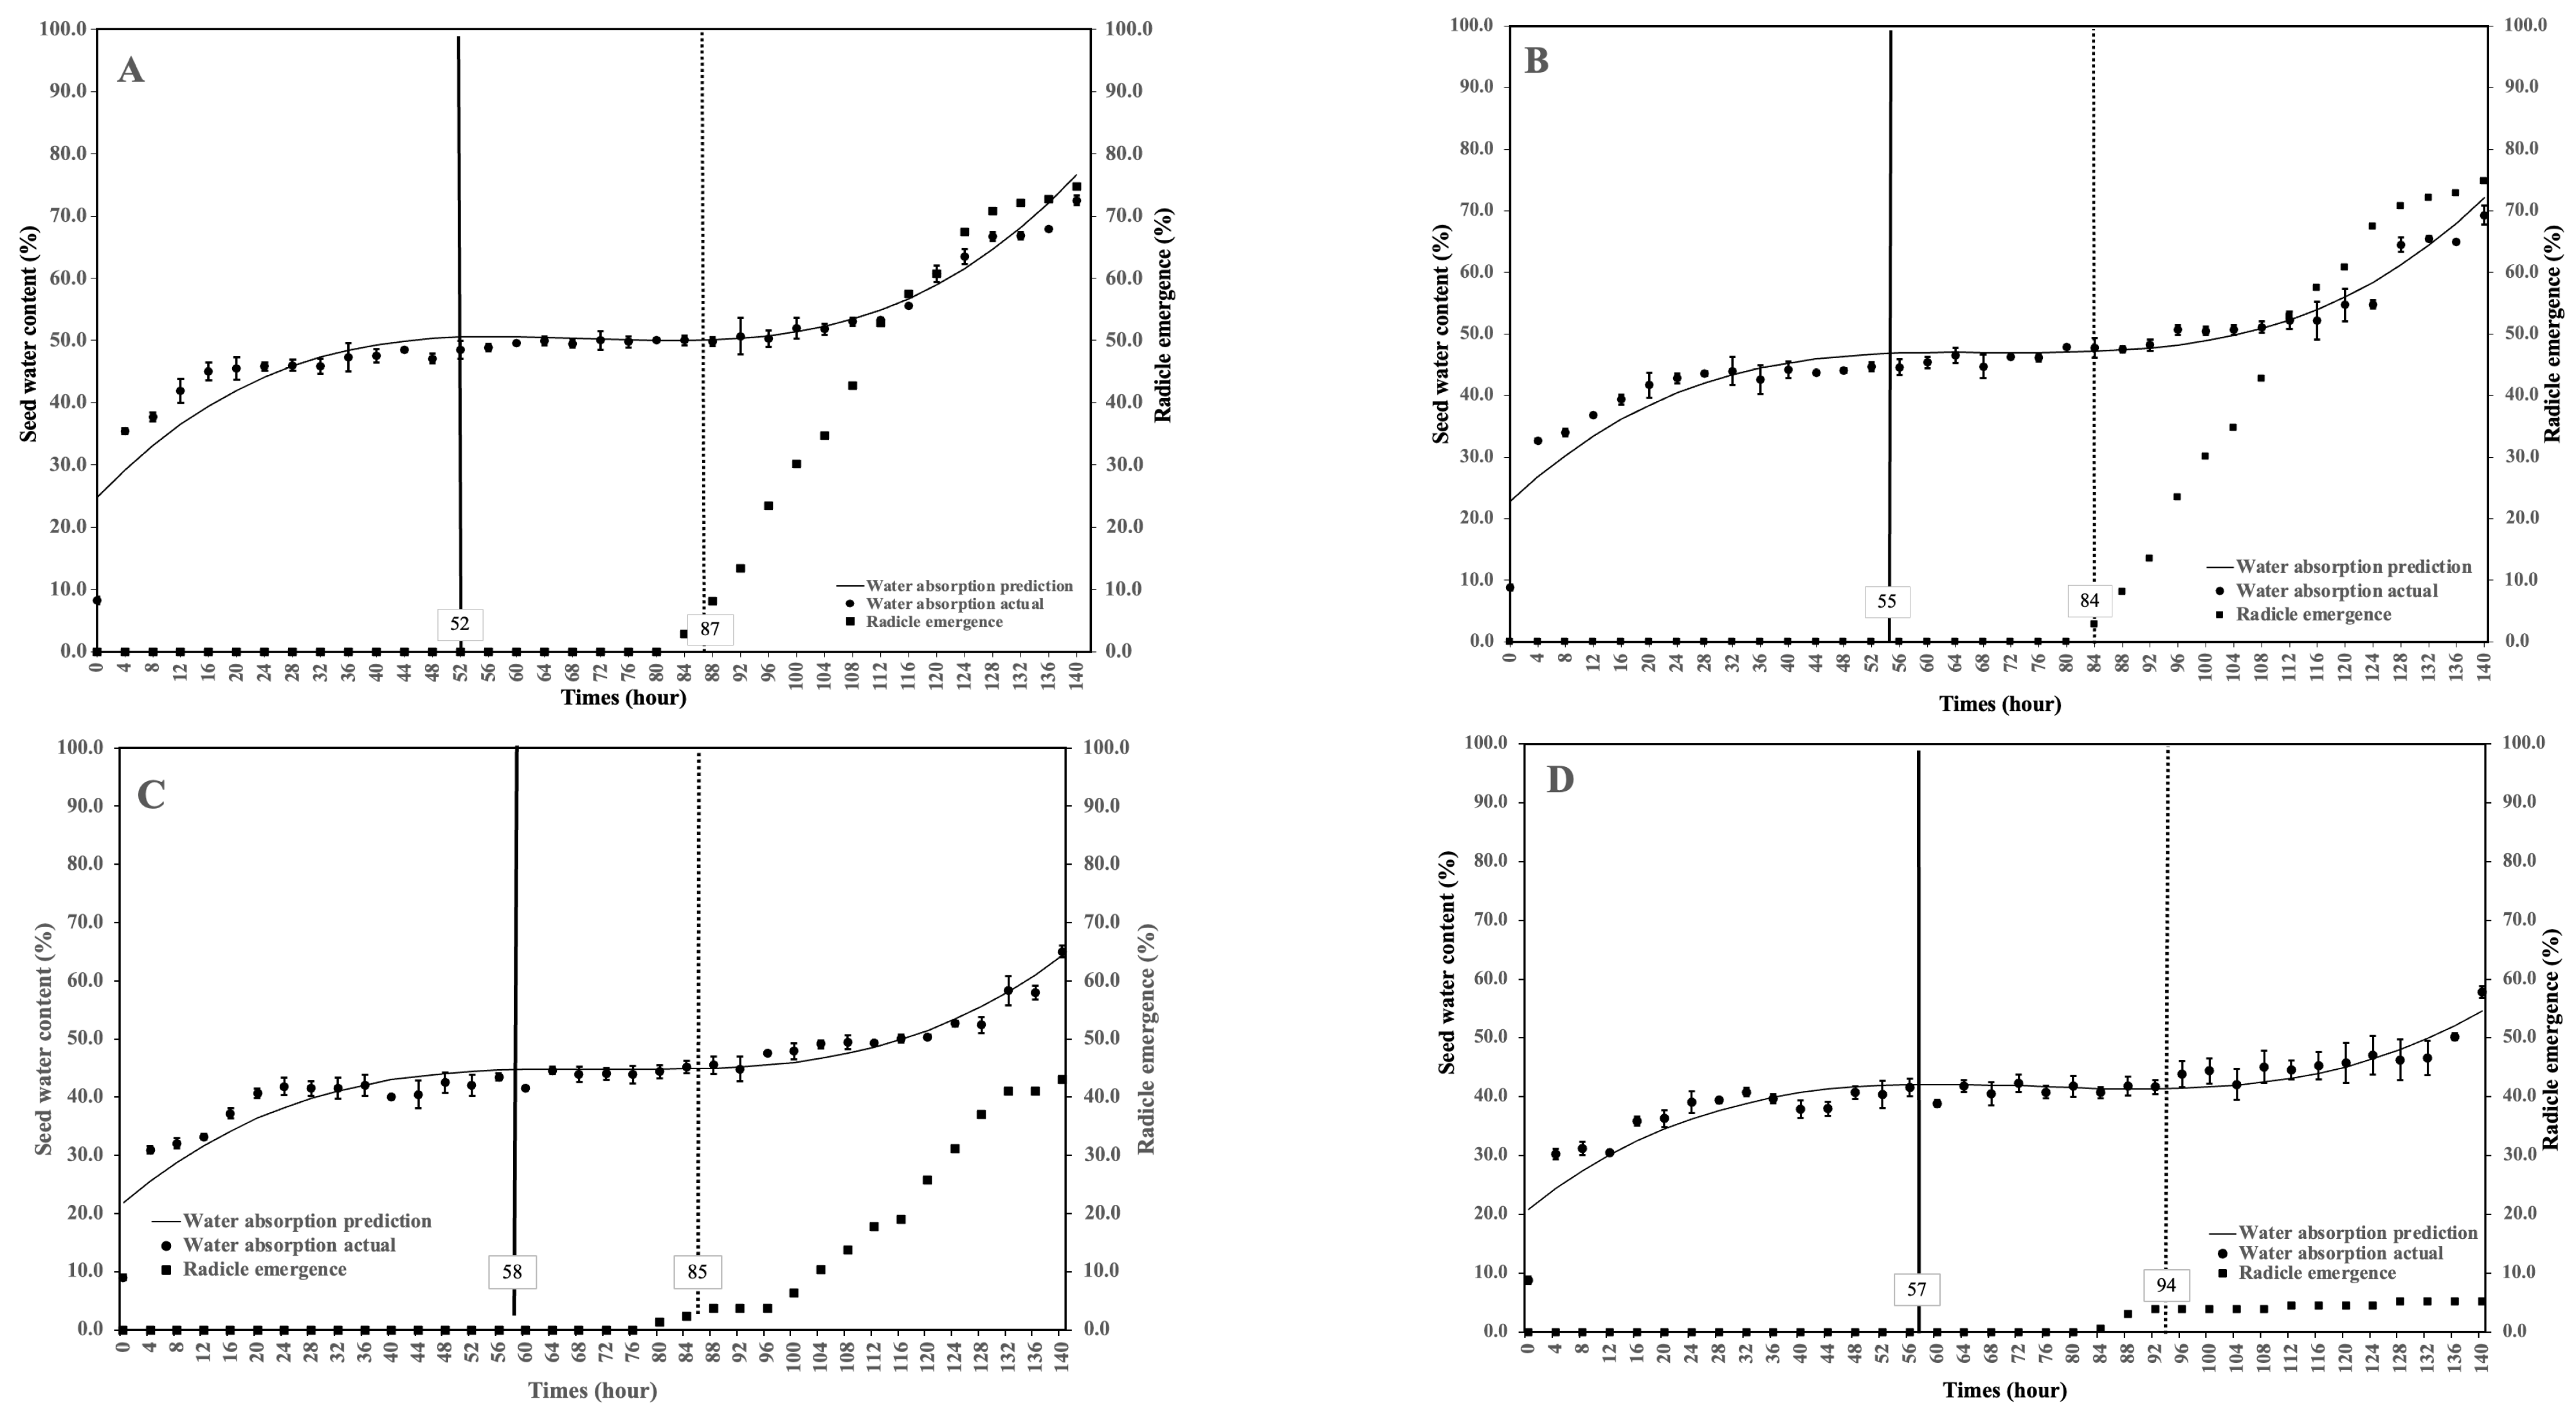
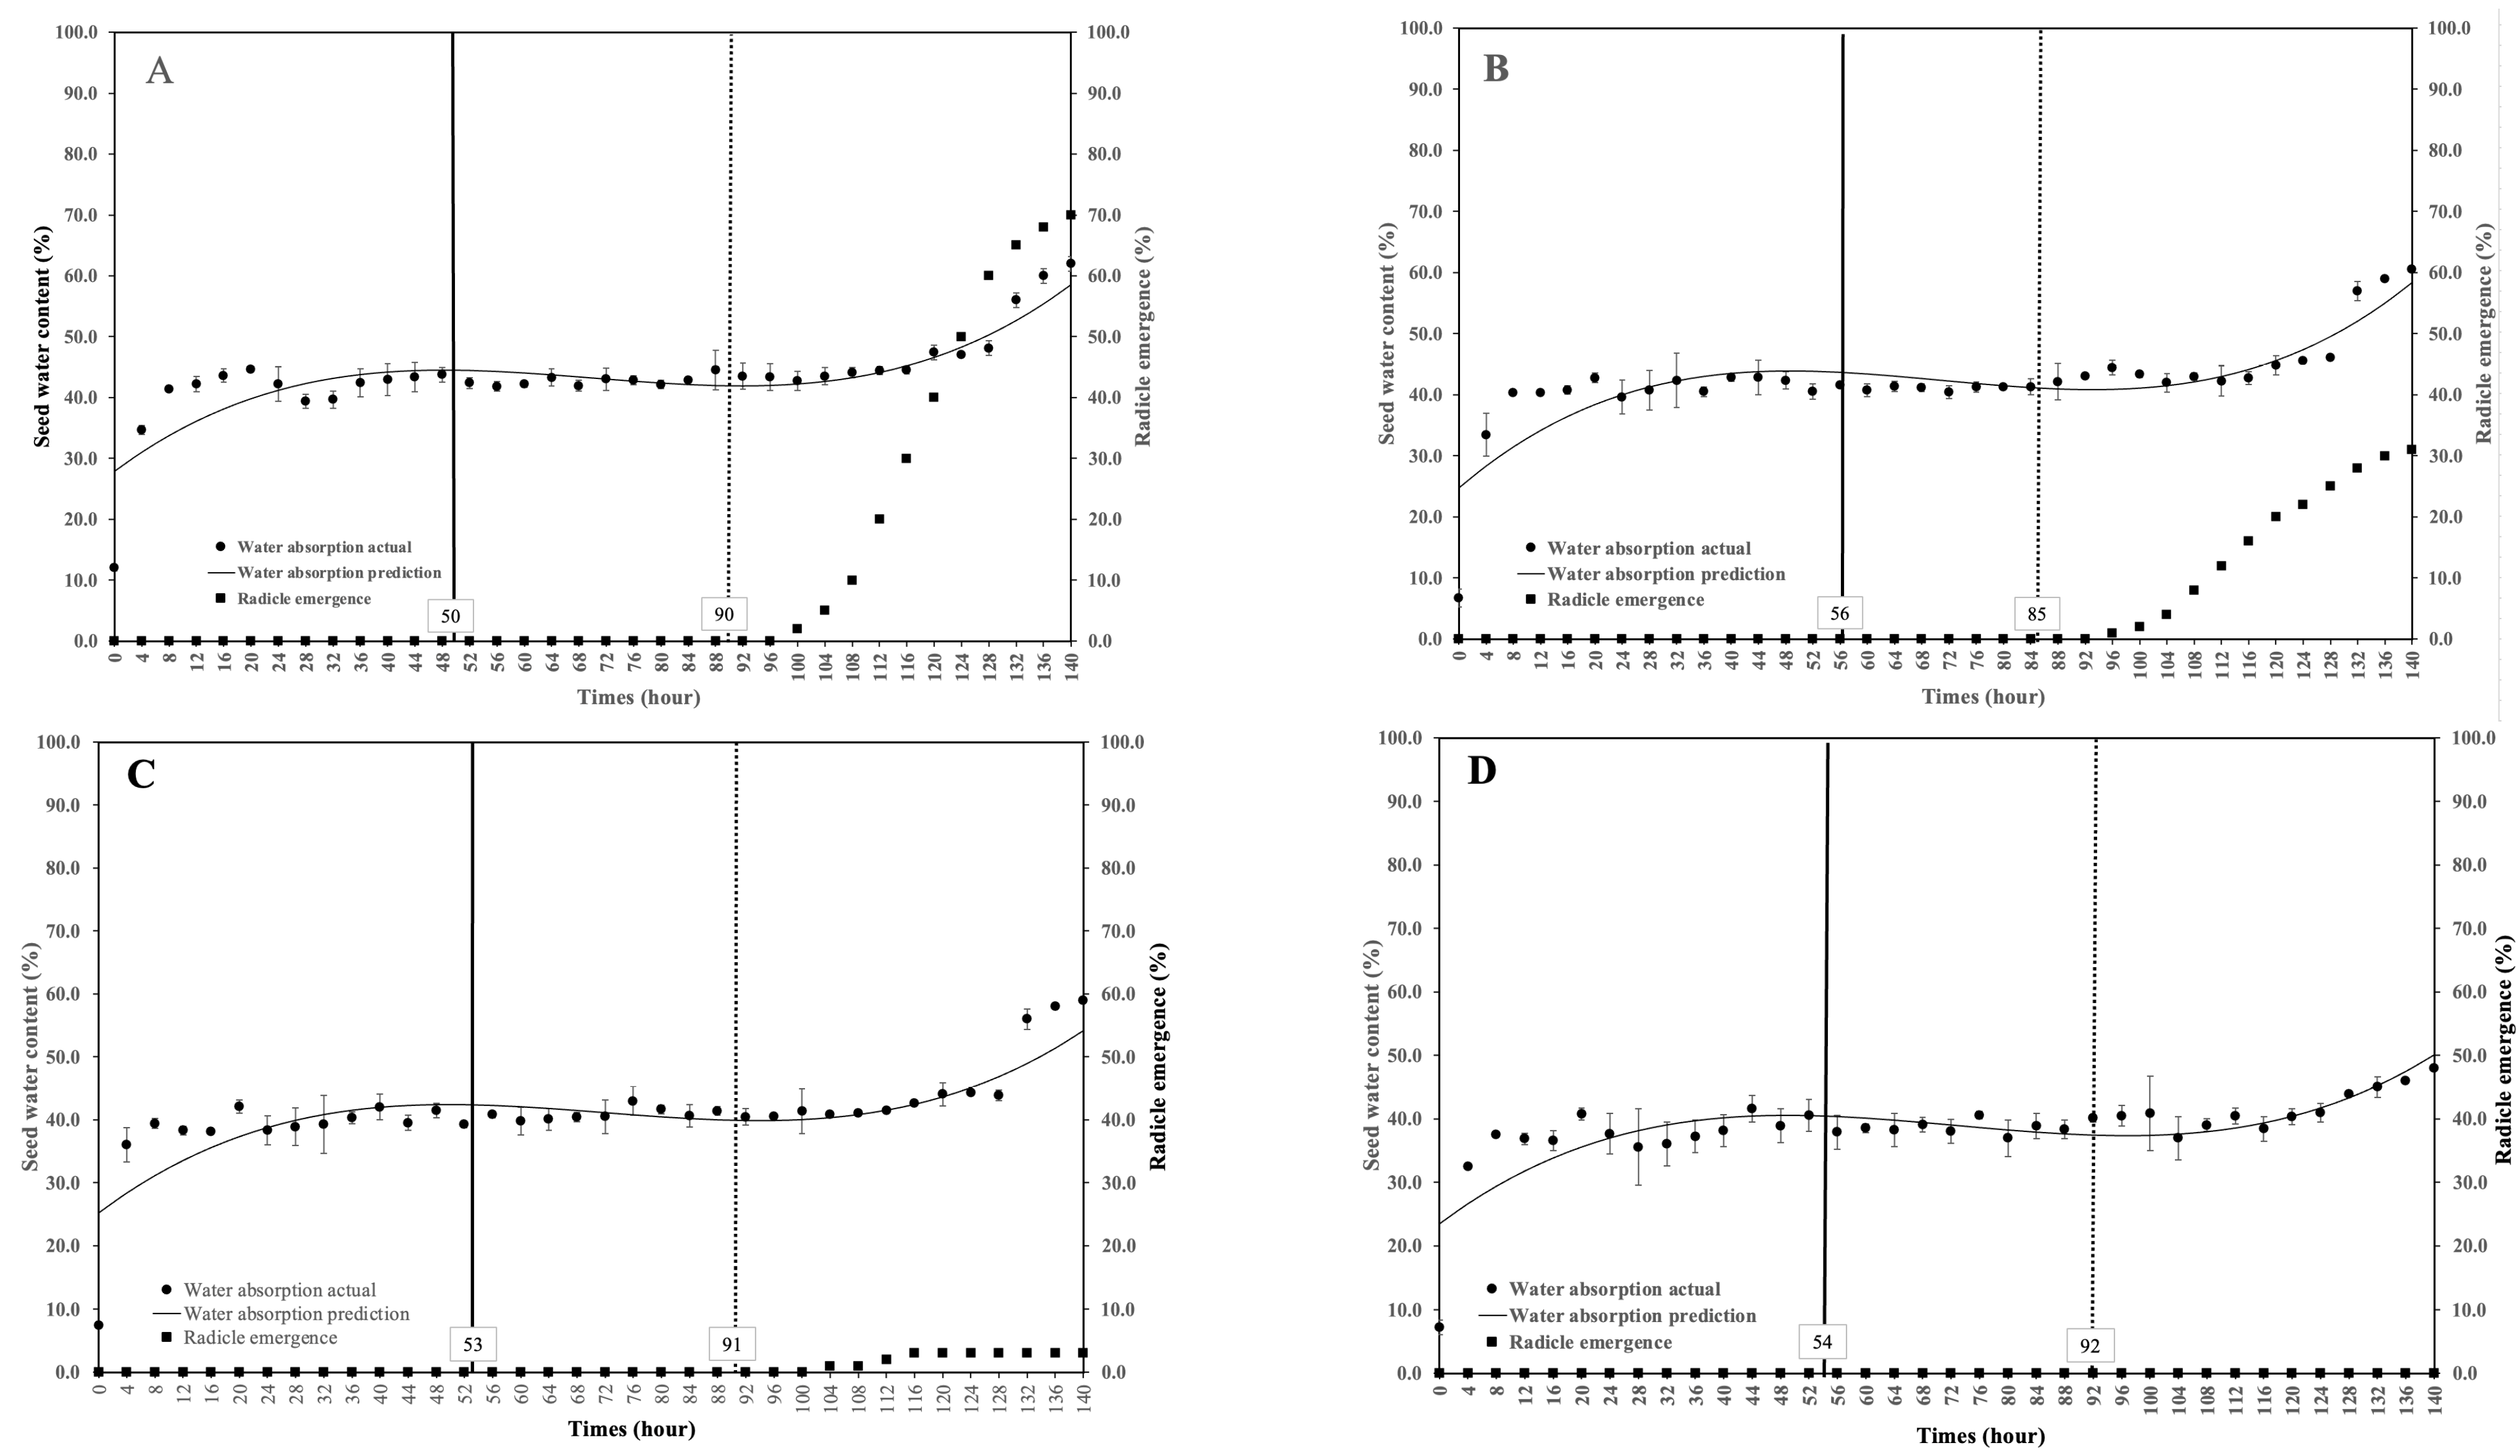
The triphasic pattern was observed at all water potential levels in eggplant seeds of the Tangguh variety (Figure 6). In contrast, in the Provita variety, the pattern did not develop at all (Figure 7). In Figure 6A (0.00 MPa), Phase I lasted approximately ~50 h, followed by Phase II extending to ~90 h, after which Phase III began and radicle emergence increased rapidly. Under mild stress (Figure 6B, −0.30 MPa), Phase I ended around ~56 h, while Phase III began near ~85 h, indicating a slight shortening of the lag phase compared to the control, although radicle emergence was reduced. Under moderate stress (Figure 6C, −1.90 MPa), Phase I lasted ~53 h and Phase III was delayed to ~91 h, with markedly lower radicle emergence. Under severe stress (Figure 6D, −4.10 MPa), Phase I remained similar (~54 h), but Phase II was prolonged and Phase III onset was delayed to ~92 h, with almost complete suppression of radicle emergence. The standard triphasic pattern was not formed in the Provita variety. Although the water content rose rapidly at the onset and then leveled off, the seed’s water content increased linearly throughout the entire imbibition process (Figure 7). Another finding from this eggplant variety was the moderate decrease in RE at each water potential level. The RE percentage obtained from water potentials of 0.00 MPa to −4.10 MPa ranged from 43.3 to 52.3%. This suggests that the Provita eggplant seed variety is resistant to osmotic stress.
Figure 6.
Imbibition and radicle emergence curves of Tangguh variety of eggplant seeds at water potentials of 0.0 MPa (A), −0.30 MPa (B), −1.90 MPa (C), and −4.1 MPa (D). Full vertical lines indicate the transition between imbibition phases 1 and 2 and dotted lines indicate the beginning of phase 3.
Figure 7.
Imbibition and radicle emergence curves of Provita variety of eggplant seeds at water potentials of 0.0 MPa (A), −0.30 MPa (B), −1.90 MPa (C), and −4.1 MPa (D).
Table 6 shows that decreasing water potential significantly affected the germination performance of the eggplant variety Tangguh (DMRT 5%). Final radicle emergence (RE) declined sharply from 70.0% at 0.00 MPa to 31.0% at −0.30 MPa and further to 3.0% at −1.90 MPa, with complete inhibition at −4.10 MPa. Time to First RE ranged from 96 to 104 h under 0.00 to −1.90 MPa, indicating generally slow germination initiation that was further delayed under moderate stress. Although T50 values numerically decreased as water potential became more negative, this trend primarily reflects the drastic reduction in total emergence rather than improved germination speed. These results indicate that Tangguh is highly sensitive to osmotic stress, particularly at water potentials ≤−1.90 MPa. In the eggplant variety Provita (Table 7), final RE decreased gradually with declining water potential, from 52.3% at 0.00 MPa to 43.3% at −4.10 MPa. Unlike Tangguh, germination was not completely inhibited even under severe stress. Time to First RE remained stable (48 h) from 0.00 to −1.90 MPa, suggesting consistent initiation of germination under mild to moderate stress, but was delayed to 60 h at −4.10 MPa. T50 increased progressively from 65 h at 0.00 MPa to 92 h at −4.10 MPa, indicating slower and less synchronized germination as water potential decreased.
Table 6.
Effects of water potential on final radicle emergence (RE), Time to First RE, and T50 in seeds of the eggplant variety Tangguh.
Table 7.
Effects of water potential on final radicle emergence (RE), Time to First RE, and T50 in seeds of the eggplant variety Provita.
4. Discussion
In general, for all commodities, the lower the water potential of the growing medium, the lower the seed’s ability to absorb water, as seen from the seed’s water content (Figure 1). At the final time of imbibition, tomato seeds exhibited greater water absorption than chili and eggplant across water potential treatments. Under optimal conditions (0.00 MPa), the tomato varieties Niki and Rempai reached 84.3% and 86.1% water content, respectively, exceeding those of chili (61.6% in Simpatik and 72.5% in Sempurna) and eggplant (62.0% in Tangguh and 78.7% in Provita). Under osmotic stress (−4.10 MPa), tomato seeds maintained water contents of 51.0% (Niki) and 55.5% (Rempai), which were generally comparable to or higher than most non-tomato cultivars. These results indicate that tomato seeds have a higher capacity for water uptake during imbibition compared with chili and eggplant, although they also show a more pronounced reduction under severe water deficit. This finding is interesting regarding the way seeds absorb water. The outer surface of the tomato seed coat is covered with fine, hair-like structures called trichomes. The anatomical structure of the seed coat plays a complex and species-specific role in water uptake [20].
The triphasic pattern does not always apply to every commodity, variety, and water potential level. From the results of this study, it appears that only chili varieties in the two varieties tested produced a triphasic pattern (Figure 2 and Figure 3). In tomato seeds, the pattern was formed only at lower water potentials of −4.10 MPa in the Niki variety (Figure 4) and the Rempai variety (Figure 5). Ref. [20] also did not find this pattern in the Cassia excelsa imbibition curve under normal conditions, but the pattern was seen when the seeds were at a water potential of −0.4 MPa. Eggplant seeds showed different results in the two varieties, where the triphasic pattern was seen in the Tangguh variety for all water potentials, while not for the Provita variety. This finding was also found in [21], where of 25 forest tree seeds tested, the triphasic pattern was only found in 11 seed types. The absence of this pattern has also been reported in several other species. Campomanesia adamantium, for example, showed a linear increase in weight from the beginning of imbibition until radicle emergence [22]. Other species that also did not exhibit a triphasic imbibition pattern include Melanoxylon brauna [23].
Overall, the results of this study indicate that the lower water potential, the later the end of phase I occurs and the longer the duration of phase II lasts. Phase II represents a plateau in water uptake following the rapid imbibition of phase I, during which pre-germinative metabolism proceeds while the radicle remains restrained. This stage is widely described as the critical window during which cellular repair, hydrolytic enzyme activity, and metabolite accumulation are initiated or intensified, without completing germination via radicle emergence [24,25,26]. The duration of phase II can vary by species and environmental conditions, and its proper execution is central to achieving improved seed vigor after subsequent dehydration and storage [25,27]. From a seed technology perspective, duration of Phase II is particularly important because it determines the seed’s capacity to tolerate environmental stress, respond to seed treatments such as priming, and maintain viability under suboptimal conditions [28,29,30,31]. Prolongation or shortening of Phase II directly influences seed vigor, uniformity of germination, and resilience to drought stress, making it a key parameter for evaluating seed quality and for developing technologies aimed at improving germination performance in water-limited environments. Environmental context during phase II (e.g., osmotic potential of the priming solution, temperature) influences the balance between continued metabolic activation and the risk of undesired radicle initiation. Several studies emphasize that priming must be controlled to avoid premature protrusion while enabling sufficient biochemical activation for improved germination later [26,32,33]. For instance, a recent study on tomato seeds (Solanum lycopersicum) indicated that osmopriming, a technique used to precondition seeds to promote germination under stress, can enhance the seeds’ performance under drought conditions. This study showed that seeds that underwent osmopriming (−1.0 MPa) displayed higher germination percentages compared to unprimed seeds when subjected to drought stress, suggesting that osmotic conditions directly impact seed viability [34,35].
Furthermore, the emergence of the radicle does not always align with the imbibition pattern results according to [3], which refers to the radicle protrusion at the end of phase II. In this study, it was observed that the emergence of the radicle tended to occur earlier, namely in the middle of phase II, except in the Tangguh eggplant variety (Figure 6). This result was also found in a study by [21], which found that only in four of 11 varieties with a triphasic pattern, germination coincided with the third phase of imbibition. There are several empirical reports that radicle emergence may occur before the canonical end of Phase II under certain conditions or in specific genotypes. For example, Ref. [36] describes a pattern where Phase II extends up to around 50–84 h depending on variety, with coleoptile elongation observed thereafter; this reflects substantial intra-species variation in the timing of the Phase II–Phase III transition and radicle-related events relative to Phase II.
Radicle emergence commonly occurs after Phase II, as per the canonical three-phase model and many priming studies; however, there is explicit evidence of genotype- and treatment-dependent variation where radicle protrusion can occur within or near the Phase II window, including mid-Phase II timing in rice and other species under certain osmotic or hormonal priming conditions [36,37]. This indicates that the standard imbibition pattern does not apply generally to every seed.
The triphasic model of seed imbibition is not universal, because its appearance likely depends on the interaction between seed structure, metabolic activation, genetic background, and environmental conditions. The model tends to be clearly visible when water uptake (Phase I), metabolic reactivation (Phase II), and radicle protrusion (Phase III) occur as temporally distinct processes. However, in some varieties, it is possible that differences in seed coat permeability, endosperm resistance, embryo growth potential, hormonal balance (e.g., ABA–GA interaction), reserve composition, and tolerance to osmotic stress may cause these processes to overlap or proceed more gradually. Under such conditions, the plateau phase may be shortened, extended, or even indistinct, resulting in a near-linear imbibition pattern rather than a well-defined triphasic curve. Therefore, the presence or absence of a clear triphasic pattern may reflect varietal-specific physiological and structural characteristics and differential stress responsiveness, although further mechanistic studies are needed to confirm these underlying causes.
5. Conclusions
Lower water potential in the growing medium reduced the seed’s ability to absorb water. A consistent triphasic imbibition pattern was observed only in chili seeds, whereas in tomato and eggplant seeds the occurrence of this pattern varied among varieties and across water potential conditions. Decreasing water potential delayed the completion of Phase I and prolonged the duration of Phase II. These findings demonstrate that the classical imbibition model cannot be universally applied to all seeds; instead, imbibition responses appear to be strongly influenced by seed type, varietal-specific physiological and structural characteristics, and the germination environment. Further mechanistic studies are needed to clarify the underlying causes of these differential responses and to support their implications for seed selection and breeding under osmotic stress conditions.
Author Contributions
A.R.: writing—original draft preparation, writing—review and editing, funding acquisition, formal analysis, data curation, conceptualization. A.Q.: writing—original draft preparation, writing—review and editing. M.R.S.: writing—original draft preparation, visualization, validation, formal analysis, data curation. O.S.I.P.: writing—original draft preparation, visualization, validation, formal analysis, data curation. A.T.: writing—original draft preparation, visualization, validation, formal analysis, data curation. P.M.S.: writing—original draft preparation, visualization. All authors have read and agreed to the published version of the manuscript.
Funding
This research was funded by Direktorat Riset dan Inovasi—Institiut Pertanian Bogor, 13120/IT3.D10/PT.01.03/P/B/2025|Institut Pertanian Bogor.
Institutional Review Board Statement
Not applicable.
Data Availability Statement
The datasets generated and/or analyzed during the current study are available from the corresponding author on reasonable request.
Acknowledgments
The authors thank the Research and Innovation Directorate—IPB University for funding the research through the young lecturer scheme on behalf of Astryani Rosyad (Contract No. 13120/IT3.D10/PT.01.03/P/B/2025). During the preparation of this manuscript, the authors used Scite_ for the purposes of analyzing citation contexts and evaluating whether referenced studies support, mention, or contrast the scientific claims discussed in this study. The authors have reviewed and edited the output and take full responsibility for the content of this publication.
Conflicts of Interest
The authors declare no conflicts of interest.
References
- Bradford, K.J. A Water Relations Analysis of Seed Germination Rates. Plant Physiol. 1990, 94, 840–849. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yousefi, A.R.; Rashidi, S.; Moradi, P.; Mastinu, A. Germination and Seedling Growth Responses of Zygophyllum fabago, Salsola kali L. and Atriplex canescens to PEG-Induced Drought Stress. Environments 2020, 7, 107. [Google Scholar] [CrossRef] [Scilit]
- Bewley, J.D.; Black, M. Seeds Physiology of Development and Germination, 3rd ed.; Plenum Press: New York, NY, USA, 2013; 445p. [Google Scholar]
- Niu, J.; Xu, M.; Zong, N.; Sun, J.; Zhao, L.; Hui, W. Ascorbic acid releases dormancy and promotes germination by an integrated regulation of abscisic acid and gibberellin in Pyrus betulifolia seeds. Physiol. Plant 2024, 176, e14271. [Google Scholar] [CrossRef] [Scilit]
- Kakar, H.A.; Ullah, S.; Shah, W.; Ali, B.; Satti, S.Z.; Ullah, R.; Muhammad, Z.; Eldin, S.M.; Ali, I.; Alwahibi, M.S.; et al. Seed Priming Modulates Physiological and Agronomic Attributes of Maize (Zea mays L.) under Induced Polyethylene Glycol Osmotic Stress. ACS Omega 2023, 8, 22788–22808. [Google Scholar] [CrossRef] [Scilit]
- Tuan, P.A.; Kumar, R.; Rehal, P.K.; Toora, P.K.; Ayele, B.T. Molecular mechanisms underlying abscisic acid/gibberellin balance in the control of seed dormancy and germination in cereals. Front. Plant Sci. 2018, 9, 362906. [Google Scholar] [CrossRef] [Scilit]
- Pompelli, M.F.; Jarma-Orozco, A.; Rodriguez-Páez, L.A. Imbibition and Germination of Seeds with Economic and Ecological Interest: Physical and Biochemical Factors Involved. Sustainability 2023, 15, 5394. [Google Scholar] [CrossRef] [Scilit]
- Soni, P.; Abdin, M.Z. Water deficit-induced oxidative stress affects artemisinin content and expression of proline metabolic genes in Artemisia annua L. FEBS Open Bio 2017, 7, 367–381. [Google Scholar] [CrossRef] [Scilit]
- Lin, J.; Shao, S.; Wang, Y.; Qi, M.; Lin, L.; Wang, Y.; Yan, X. Germination responses of the halophyte Chloris virgata to temperature and reduced water potential caused by salinity, alkalinity and drought stress. Grass Forage Sci. 2016, 71, 507–514. [Google Scholar] [CrossRef] [Scilit]
- Khetsha, Z.; van der Watt, E.; Masowa, M.; Legodi, L.; Satshi, S.; Sadiki, L.; Moyo, K. Phytohormone-Based Biostimulants as an Alternative Mitigating Strategy for Horticultural Plants Grown Under Adverse Multi-Stress Conditions: Common South African Stress Factors. Caraka Tani J. Sustain. Agric. 2024, 39, 167–193. [Google Scholar] [CrossRef] [Scilit]
- Motti, R. The Solanaceae Family: Botanical Features and Diversity; Springer International Publishing: Cham, Switzerland, 2021; pp. 1–9. [Google Scholar]
- Megersa, H.G. Potential Effects of Salt Stress on Selected Solanaceous Crops (Tomato (Solanum esculentum L.) and Hot Pepper (Capsicum annuum L.)) Production. J. Agric. Sci. Food Res. 2022, 13, 1–6. [Google Scholar]
- Pessoa, H.P.; de Carvalho Rocha, J.R.D.A.S.; Alves, F.M.; Copati, M.G.F.; Dariva, F.D.; da Silva, L.J.; Carneiro, P.C.; Gomes, C.N. Multi-trait selection of tomato introgression lines under drought-induced conditions at germination and seedling stages. Acta Sci. Agron. 2022, 44, e55876. [Google Scholar] [CrossRef] [Scilit]
- Barris, S.; Toumi, M.; Belkebir, A. Effect of osmotic and salt stresses on germination and phenolic compounds of Eruca vesicaria subs. sativa L. Res. Sq. 2022. [Google Scholar] [CrossRef] [Scilit]
- Lei, C.; Bagavathiannan, M.; Wang, H.; Sharpe, S.M.; Meng, W.; Yu, J. Osmopriming with Polyethylene Glycol (PEG) for Abiotic Stress Tolerance in Germinating Crop Seeds: A Review. Agronomy 2021, 11, 2194. [Google Scholar] [CrossRef] [Scilit]
- Radić, V.; Balalić, I.; Cvejić, S.; Jocić, S.; Marjanović-Jeromela, A.; Miladinović, D. Drought effect on maize seedling development. Ratar. Port. 2018, 55, 135–138. [Google Scholar] [CrossRef] [Scilit]
- Mexal, J.; Fisher, J.T.; Osteryoung, J.; Reid, C.P.P. Oxygen Availability in Polyethylene Glycol Solutions and Its Implications in Plant-Water Relations. Plant Physiol. 1975, 55, 20–24. [Google Scholar] [CrossRef] [Scilit]
- ISTA. International Rules for Seed Testing 2018. Available online: https://www.tarimorman.gov.tr/BUGEM/TTSM/Belgeler/Duyuru%20Belgeleri/ISTA%20Rules%202018.pdf (accessed on 19 April 2025).
- Bewley, J.D.; Bradford, K.J.; Hilhorst, H.W.M.; Nonogaki, H. Seeds: Physiology of Development, Germination and Dormancy, 3rd ed.; Springer: New York, NY, USA, 2008. [Google Scholar] [CrossRef] [Scilit]
- Upretee, P.; Bandara, M.S.; Tanino, K.K. The Role of Seed Characteristics on Water Uptake Preceding Germination. Seeds 2024, 3, 559–574. [Google Scholar] [CrossRef] [Scilit]
- Pereira, W.V.S.; José, A.C.; Tonetti, O.A.O.; de Melo, L.A.; Faria, J.M.R. Imbibition curve in forest tree seeds and the triphasic pattern: Theory versus practice. S. Afr. J. Bot. 2022, 144, 105–114. [Google Scholar] [CrossRef] [Scilit]
- Dresch, D.M.; de Quintão Scalon, S.P.; Elisa Masetto, T.; do Carmo Vieira, M. Germinação e vigor de sementes de gabiroba em função do tamanho do fruto e semente. Pesqui. Agropecu. Trop. 2013, 43, 262–271. [Google Scholar] [CrossRef] [Scilit]
- Flores, A.V.; Borges, E.E.D.L.E.; Guimarães, V.M.; Da Mata Ataíde, G.; Castro, R.V.O. Germinação de sementes de Melanoxylon brauna schott em diferentes temperaturas. Rev. Árvore 2014, 38, 1147–1154. [Google Scholar] [CrossRef] [Scilit]
- Seethalakshmi, S.; Umarani, R.; Maduraimuthu, D. Gibberellic Acid Biosynthesis During Dehydration Phase of Priming Increases Seed Vigour of Tomato. Plant Growth Regul. 2022, 97, 255–262. [Google Scholar] [CrossRef] [Scilit]
- Pedrini, S.; Balestrazzi, A.; Madsen, M.D.; Bhalsing, K.; Hardegree, S.P.; Dixon, K.W.; Kildisheva, O.A. Seed enhancement: Getting seeds restoration-ready. Restor. Ecol. 2020, 28, S266–S275. [Google Scholar] [CrossRef] [Scilit]
- Raj, A.B.; Raj, S.K. Seed priming: An approach towards agricultural sustainability. J. Appl. Nat. Sci. 2019, 11, 227–234. [Google Scholar] [CrossRef] [Scilit]
- Lechowska, K.; Kubala, S.; Wojtyla, Ł.; Nowaczyk, G.; Quinet, M.; Lutts, S.; Garnczarska, M. New Insight on Water Status in Germinating Brassica napus Seeds in Relation to Priming-Improved Germination. Int. J. Mol. Sci. 2019, 20, 540. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gama, G.F.V.; Brum, L.B.T.L.; Martins, M.S.; da Silva, L.J.; dos Dias, D.C.F.S. Silicon in wheat crop under water limitation and seed tolerance to water stress during germination. Rev. Ceres 2021, 68, 360–367. [Google Scholar] [CrossRef] [Scilit]
- Guo, M.; Zong, J.; Zhang, J.; Wei, L.; Wei, W.; Fan, R.; Zhang, T.; Tang, Z.; Zhang, G. Effects of temperature and drought stress on the seed germination of a peatland lily (Lilium concolor var. megalanthum). Front. Plant Sci. 2024, 15, 1462655. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wu, L.Y.; Yan, J.; Huang, Z.W.; Wan, Y.H.; Zhu, W.M. Solid matrix priming improves cauliflower and broccoli seed germination and early growth under the suboptimal temperature conditions. PLoS ONE 2022, 17, e0275073. [Google Scholar] [CrossRef] [Scilit]
- Tu, K.; Cheng, Y.; Pan, T.; Wang, J.; Sun, Q. Effects of Seed Priming on Vitality and Preservation of Pepper Seeds. Agriculture 2022, 12, 603. [Google Scholar] [CrossRef] [Scilit]
- Gueridi, S.; Boucelha, L.; Abrous-Belbachir, O.; Djebbar, R. Effects of hormopriming and pretreatment with gibberellic acid on fenugreek (Trigonella foenum-graecum L.) seed germination. Acta Bot. Croat. 2024, 83, 135–144. [Google Scholar] [CrossRef] [Scilit]
- Manhone, P.R.; Lopes, J.C.; Alexandre, R.S.; Lima, P.A.M.; Lopes, S.O.; Mengarda, L.H.G.; Mello, T. Plant growth regulators and mobilization of reserves in imbibition phases of yellow passion fruit. Braz. J. Biol. 2024, 84, e273999. [Google Scholar] [CrossRef] [Scilit]
- da Silva, P.B.; Vaz, T.A.A.; Acencio, M.L.; Bovolenta, L.A.; Hilhorst, H.W.M.; da Silva, E.A.A. Can Osmopriming Induce Cross-Tolerance for Abiotic Stresses in Solanum paniculatum L. Seeds? A Transcriptome Analysis Point of View. Seeds 2023, 2, 382–393. [Google Scholar] [CrossRef] [Scilit]
- Sano, N.; Verdier, J. The re-establishment of desiccation tolerance in germinated tomato (Solanum lycopersicum) seeds. Seed Sci. Res. 2024, 34, 77–85. [Google Scholar] [CrossRef] [Scilit]
- Cheng, J.; Wang, L.; Zeng, P.; He, Y.; Zhou, R.; Zhang, H.; Wang, Z. Identification of genes involved in rice seed priming in the early imbibition stage. Plant Biol. 2017, 19, 61–69. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Adhikari, B.; Dhital, P.R.; Ranabhat, S.; Poudel, H. Effect of seed hydro-priming durations on germination and seedling growth of bitter gourd (Momordica charantia). PLoS ONE 2021, 16, e0255258. [Google Scholar] [CrossRef] [Scilit] [PubMed]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.