


Abstract
Autophagy is an evolutionarily preserved intracellular degradation process pivotal in maintaining proteostasis, mitochondrial homeostasis, and metabolic equilibrium, all of which are dysregulated with aging. Aberrant autophagy has been recognized as a hallmark of human aging and age-related diseases, including neurodegeneration, metabolic dysfunction, cardiovascular diseases, and cancer. Bioactive natural compounds derived from plants, foods, and marine organisms have emerged as potent modulators of autophagy, offering a promising strategy to counteract aging and promote healthy lifespan. Mechanistically, these compounds regulate autophagy by modulating key signaling pathways, such as AMPK, PI3K/AKT/mTOR, SIRT1, and FOXO, while also alleviating oxidative stress, inflammation, and mitochondrial dysfunction. Natural compounds like polyphenols, flavonoids, alkaloids, terpenoids, and carotenoids exhibit dual roles by restoring age-related suppressed autophagic flux and inhibiting excessive autophagy-induced cell death. In this review, we provide a comprehensive overview of the molecular mechanisms through which bioactive natural compounds modulate autophagy and impact human aging and longevity. We discuss both experimental and clinical evidence supporting their geroprotective effects, limitations regarding bioavailability and dose-dependent effects, and prospects for the utilization of autophagy-targeting natural products in aging intervention strategies.
1. Introduction
Autophagy is a lysosome-dependent catabolic process that degrades damaged organelles, misfolded proteins, and toxic aggregates, thus maintaining metabolic homeostasis and cellular integrity throughout the lifespan [1]. Aging is a multifactorial biological process characterized by a gradual decline in cellular, tissue, and organ function, eventually leading to an increased risk of chronic diseases and death [2]. At the cellular level, aging is driven by the accumulation of molecular damage, impaired protein quality control, mitochondrial dysfunction, oxidative stress, and chronic low-grade inflammation [3]. Evidence from various sources supports the view that autophagic flux declines with age in many tissues, including the brain, liver, skeletal muscle, and cardiovascular system [4]. Age-related impairment in autophagy leads to cellular senescence, decreased stress resilience, and functional decline, all of which accelerate the aging process and contribute to the development of age-related diseases [5]. Experimental studies in model organisms have revealed that genetic or pharmacological activation of autophagy can extend lifespan and promote health span, suggesting autophagy as a therapeutic target for aging intervention [6]. Consequently, strategies to restore or optimize autophagic flux have gained significant attention in the field of aging research.
In recent decades, bioactive natural compounds from food sources, medicinal plants, and marine organisms have emerged as powerful and physiologically relevant modulators of autophagy [7]. These molecules often exhibit multitargeted actions that are closely aligned with the biological complexity of aging. Generally, bioactive natural compounds act by reestablishing dysfunctional autophagic processes, thus modulating cellular resilience to age-related stress rather than inducing excessive autophagy [8]. Polyphenols, flavonoids, alkaloids, terpenoids, and carotenoids are known to regulate autophagy by modulating the activity of key signaling pathways, such as AMPK, PI3K/AKT/mTOR, SIRT1, and FOXO, which are also crucial in the regulation of aging and lifespan [9].
In addition to their autophagy-modulating properties, natural products possess other geroprotective effects, including the reduction in oxidative stress, inhibition of chronic inflammation, improvement of mitochondrial quality control, and maintenance of metabolic homeostasis [10]. These coordinated effects position bioactive natural compounds as promising agents for promoting healthy aging and delaying the onset of age-related diseases. However, despite promising experimental data, several challenges still need to be addressed for translating these molecules into clinically relevant anti-aging interventions, including bioavailability, dosage specificity, and tissue-targeted effects. In this review, we explore the molecular mechanisms by which bioactive natural compounds regulate autophagy and their implications for human aging and longevity. By integrating molecular, experimental, and emerging clinical evidence, we aim to provide a comprehensive framework to better understand how the regulation of autophagy by natural products can be leveraged to promote healthy aging and extend lifespan.
2. Molecular Mechanisms of Autophagy in Human Aging and Longevity Control
Autophagy is a highly regulated, lysosome-dependent catabolic process essential for maintaining cellular quality control and adaptive stress responses, both of which are key determinants of human aging and longevity. At the molecular level, autophagy is induced in response to nutrient deprivation, oxidative stress, and metabolic imbalances through the intricate orchestration of evolutionarily conserved signaling pathways [11]. Central to its regulation is the balance between anabolic and catabolic signals, with the AMPK and PI3K/AKT/mTOR signaling pathways playing a dominant role [12]. AMP-activated protein kinase (AMPK) is an energy sensor that triggers autophagy through the phosphorylation of ULK1 and the inhibition of mTORC1 activity under low-energy conditions [13]. On the other hand, mTORC1 acts as a negative regulator of autophagy by blocking the activation of the ULK1 complex under nutrient-rich conditions. Dysregulation of autophagy is associated with the aging process, including persistent activation of mTORC1 and blunted AMPK signaling, leading to chronic suppression of autophagy and the accumulation of damaged cellular components [14]. Reinstating AMPK activity or inhibiting mTOR signaling has been shown to enhance autophagic flux and extend lifespan in various model systems. Figure 1 explores the evolutionarily conserved nutrient-sensing and stress–response pathways that regulate autophagy and influence aging and longevity.
Figure 1.
Evolutionarily conserved signaling mechanisms regulated by autophagy. Low energy, oxidative stress, or food deprivation activates AMPK by decreasing ATP and increasing cellular stress signals. Activated AMPK phosphorylates ULK1, forming the active complex and autophagosomes. AMPK also reduces mTORC1 activity, releasing autophagy inhibitory effects. Nutrient-rich circumstances and aging promote PI3K/AKT signaling and mTORC1 activation. ULK1 activation and autophagosome formation are blocked by active mTORC1, suppressing autophagic flow. Age-related chronic mTORC1 activation reduces AMPK signaling, mitochondrial malfunction, protein and organelle degradation, and cellular damage. AMPK-mTORC1 balance as a major autophagy regulator. Experimental therapies like AMPK activators and mTORC1 inhibitors increase autophagic flux, lysosomal function, mitochondrial quality control, and cellular health. These conserved signaling pathways regulate autophagy, cellular homeostasis, and longevity across species by integrating energy status, redox balance, and nutrient sensing.
The Sirtuin family of proteins, particularly SIRT1, modulates longevity by deacetylating key autophagy-related proteins, including ATG5, ATG7, and LC3, thereby promoting the formation and maturation of autophagosomes [15]. SIRT1 also regulates transcription factors like FOXO and PGC-1α, which coordinate autophagy, mitochondrial biogenesis, and antioxidant defense pathways [16]. The age-related decline in NAD+ levels impairs SIRT1 activity, impairing autophagy and accelerating cellular aging. Transcription factor EB (TFEB) is a master regulator of lysosomal biogenesis and autophagy-related gene expression at the transcriptional level [17]. The reduced nuclear translocation of TFEB with age impairs lysosomal function and autophagic degradation [18]. Additionally, an excess of reactive oxygen species and chronic inflammation can inhibit autophagy through post-translational modifications of autophagy-related proteins. Collectively, the dysregulation of autophagy results in the accumulation of protein aggregates, dysfunctional mitochondria, and genomic instability, all of which contribute to aging and limit lifespan. Targeting these molecular checkpoints to restore balanced autophagic activity is a promising strategy to promote healthy aging and extend longevity (Figure 2).
Figure 2.
Sirtuin-mediated regulation of autophagy and longevity in molecular interconnections and aging impairments. (A) Young Cell with Efficient Autophagy: In young cells, sufficient NAD+ levels support SIRT1 activity, leading to deacetylation of autophagy-related proteins such ATG5, ATG7, and LC3. A post-translational change boosts autophagosome production and maturation. SIRT1 upregulates genes involved in autophagy, mitochondrial biogenesis, and antioxidant defense by activating transcriptional regulators such FOXO and PGC-1α. While translocating to the nucleus, TFEB stimulates lysosomal biogenesis and autophagy gene expression, promoting autophagic flux. These coordinated molecular interactions preserve mitochondrial quality, redox balance, genomic stability, and cellular health, promoting longevity. (B) Aged Cell with Impaired Autophagy: As we age, NAD+ depletion reduces SIRT1 activity, causing autophagy-related protein acetylation and decreased autophagy initiation. Decreased FOXO, PGC-1α, and TFEB activation reduces autophagy, lysosomal, and antioxidant gene expression. Protein clumps, reactive oxygen species, mitochondrial malfunction, and genetic instability further reduce autophagic flow. Chronic inflammation and post-translational inhibition worsen lysosomal dysfunction. These molecular disruptions cause cellular quality control issues, faster aging, and shorter lifespans.
Figure 1: The central molecular pathways regulate autophagy and their impact on human aging and longevity. The AMPK pathway serves as a principal autophagy enhancer in low-energy settings by detecting increased AMP levels and activating the ULK1 complex to commence autophagosome production. The mTORC1 pathway serves as a principal inhibitor of autophagy, combining signals from nutrients, glucose, amino acids, and insulin through PI3K-AKT signaling to decrease ULK1 activation in nutrient-abundant environments. Sirtuins and NAD+ signaling, especially SIRT1, enhance autophagy by deacetylating essential autophagy proteins ATG5, ATG7, and LC3, while also facilitating mitochondrial homeostasis, antioxidant defenses, and longevity-related transcriptional programs via FOXO and PGC-1α. The reduction of NAD+ with age restricts these protective benefits. TFEB-mediated lysosomal regulation governs the transcription of autophagy and lysosomal genes, augmenting lysosome formation and degradative capacity vital for effective autophagic flux. Inhibitory factors, such as increased reactive oxygen species and chronic inflammation, hinder the functionality of autophagy proteins and lysosomal breakdown. The coordinated regulation of these pathways maintains cellular homeostasis, mitigates aging-related damage, and promotes longevity.
3. Bioactive Natural Products as Autophagy Modulators in Aging and Longevity Control
Bioactive natural compounds have emerged as attractive candidates for autophagy modulation with implications for human aging and lifespan regulation [8]. Unlike conventional single-target synthetic drugs, natural products often exhibit pleiotropic actions that align with the complex and multifactorial nature of aging. Their ability to modulate autophagy contextually, restoring impaired autophagic flux rather than causing unregulated induction of autophagy, positions them as potential candidates for promoting healthy aging and lifespan extension [19]. Decreased autophagy is a hallmark of aging, resulting in the accumulation of damaged proteins, dysfunctional mitochondria, and metabolic disturbances [4]. Bioactive natural compounds counteract these changes by fine-tuning key molecular pathways involved in autophagy regulation, including AMPK, PI3K/AKT/mTOR, SIRT1, FOXO, and TFEB [20]. These compounds act primarily as modulators of autophagy rather than as strong activators, avoiding both insufficient clearance and excessive cytotoxicity associated with dysregulated autophagy. Major groups of compounds involved in autophagy modulation include polyphenols, flavonoids, alkaloids, terpenoids, and carotenoids, which are found in dietary components, medicinal plants, and marine organisms (Figure 3).
Figure 3.
Modulation of autophagy in aging by bioactive natural products. Section 1 demonstrates the age-associated reduction in autophagy, resulting in the accumulation of damaged or misfolded protein aggregates, mitochondrial malfunction, and metabolic dysregulation in older cells. Section 2 delineates principal sources and categories of bioactive natural compounds, encompassing dietary polyphenols and flavonoids, plant-derived alkaloids and terpenoids, and marine-derived carotenoids, all of which jointly influence autophagy control. Section 3 illustrates the principal molecular pathways influenced by these substances, wherein the activation of AMPK and SIRT1 promotes autophagy via phosphorylation and deacetylation processes, while the inhibition of the PI3K/AKT/mTOR pathway alleviates restrictions on autophagic signaling. Transcriptional regulation by TFEB and FOXO enhances the expression of genes associated with autophagy and lysosomes, hence reinstating autophagic flow. Section 4 illustrates the results of balanced autophagy modulation, encompassing enhanced proteostasis, preservation of healthy mitochondria, and avoidance of cellular malfunction.
Polyphenols represent one of the most extensively studied groups of natural compounds with autophagy modulatory effects (Table 1). Polyphenols, such as resveratrol, curcumin, epigallocatechin gallate, and quercetin, are abundant in fruits, vegetables, tea, coffee, and red wine, and have been shown to significantly impact cellular aging pathways [21]. Mechanistically, polyphenols enhance AMPK and SIRT1 signaling, while also inhibiting mTORC1 activity, thus promoting balanced autophagy induction and autophagic flux [22]. Additionally, their antioxidants and anti-inflammatory properties help reduce oxidative and inflammatory stress, which can otherwise impair autophagy during aging. The combined effects of polyphenols promote mitochondrial quality control, proteostasis, and metabolic flexibility, contributing to improved cellular resilience and longevity [23].
Resveratrol, a stilbene polyphenol, primarily acts as a chain-breaking radical-trapping antioxidant. The activity encompasses hydrogen atom transfer and successive proton-loss electron transfer processes, enabled by phenolic hydroxyl groups [24]. Its activity is affected by solvent polarity and pH, exhibiting increased reactivity under slightly alkaline conditions. With moderate lipophilicity, it divides into membranes, scavenging peroxyl radicals and modulating superoxide-derived species [25]. While not a traditional enzymatic antioxidant, it enhances the expression of endogenous ROS-detoxifying enzymes and indirectly facilitates the regeneration of glutathione and α-tocopherol through Nrf2 activation [26]. Curcumin, a diarylheptanoid, functions as a radical-scavenging and metal-chelating antioxidant. It experiences hydrogen atom donation and electron transfer, with keto-enol tautomerism affecting solvent-dependent reactivity [27]. Its lipophilicity promotes membrane localization and the neutralization of lipid peroxyl radicals. Curcumin additionally augments glutathione biosynthesis and bolsters redox enzyme systems [28]. EGCG, quercetin, fisetin, kaempferol, apigenin, luteolin, genistein, and chlorogenic acid are derivatives of flavonoids or phenolic acids that primarily act as radical-trapping antioxidants via hydrogen atom transfer and electron transfer pathways, influenced by hydroxyl patterns and ring conjugation [29,30]. Their reactivity fluctuates with pH and polarity, affecting the scavenging of superoxide, hydroxyl, and nitrogen-centered radicals. Various chelate transition metals indirectly promote the regeneration of glutathione, coenzyme Q10, and α-tocopherol through redox cycling networks [31].
Table 1.
Major Polyphenols and their autophagy modulation in aging and longevity regulation.
Flavonoids, a subclass of polyphenols, encompass compounds like luteolin, apigenin, kaempferol, and myricetin, which are found in fruits, vegetables, and medicinal herbs [42]. Flavonoids regulate autophagy by modulating both upstream signaling pathways and the transcriptional regulation of autophagy-related genes [43]. Many flavonoids facilitate AMPK activation and inhibit PI3K/AKT signaling, leading to mTOR inhibition and controlled induction of autophagy [44]. Simultaneously, flavonoids regulate FOXO and TFEB transcription factors, promoting lysosomal biogenesis and maintaining efficient autophagic degradation [17]. These effects are particularly relevant in aging tissues, such as the brain and skeletal muscle, where autophagy dysfunction contributes to functional decline. Table 2 presents the predominant flavonoids and their modulation of autophagy in the regulation of aging and longevity.
Flavonoids including luteolin, apigenin, kaempferol, myricetin, fisetin, quercetin, naringenin, hesperidin, baicalein, and genistein are polyphenolic radical-trapping antioxidants (RTAs) distinguished by phenolic hydroxyl groups that facilitate hydrogen atom transfer and single-electron transfer mechanisms [45]. Their antioxidant activity often occurs through hydrogen atom transfer, consecutive proton-loss electron transfer, or single-electron transfer followed by proton transfer, contingent upon hydroxyl substitution patterns and conjugation across the C ring [46]. Ortho-dihydroxy structures, especially in quercetin, luteolin, and baicalein, augment the stability of phenoxyl radicals via resonance, hence enhancing the efficacy in scavenging peroxyl (ROO•), superoxide (O2•−), hydroxyl (•OH), and nitrogen-centered radicals such as •NO and •NO2 [47]. Their reactivity is contingent upon pH, as deprotonation under somewhat alkaline conditions amplifies electron-donating capacity [48]. The polarity of solvents affects the stability of radicals and their bioavailability. Lipophilicity differs: flavonols like quercetin and kaempferol demonstrate partial membrane partitioning, facilitating the prevention of lipid peroxidation, while glycosylated hesperidin is more hydrophilic and mostly functions in aqueous environments [49]. In addition to direct radical scavenging, certain flavonoids enhance the expression of endogenous antioxidant enzymes such as superoxide dismutase, catalase, and glutathione peroxidase through Nrf2 activation [50]. Numerous individuals engage indirectly in the breakdown of enzymatic ROS/RNS by maintaining glutathione reserves and promoting redox cycling. Quercetin and luteolin can restore α-tocopherol in lipid environments, whereas other compounds facilitate the regeneration of glutathione, coenzyme Q10, and lipoic acid redox states [51].
Table 2.
Principal flavonoids and their modulation of autophagy in the regulation of aging and longevity.
Alkaloids, a diverse class of nitrogen-containing compounds, are widely distributed in plants, many of which possess medicinal properties and play a significant role in regulating aging through autophagy [59]. Alkaloids modulate aging-related autophagy chiefly by adjusting the AMPK-mTOR pathway, altering stress factors like ROS and inflammation, and modulating reforming transcriptional or epigenetic mechanisms that govern autophagy gene expression [60]. Significantly, many alkaloids seem to normalize autophagic flux instead of only enhancing autophagy, a characteristic that is mechanistically associated with good aging and longevity regulation [61]. Alkaloids and related nitrogenous compounds such as berberine, caffeine, and spermidine have been shown to modulate lifespan pathways by enhancing autophagic capacity. Spermidine has garnered attention for its ability to induce autophagy through epigenetic regulation, including inhibition of histone acetyltransferases and activation of autophagy gene expression [62]. Berberine activates AMPK signaling, improves mitochondrial function, and reduces chronic inflammation, indirectly promoting autophagy during aging [63]. These properties position alkaloids as regulators of autophagy and metabolic health. Important alkaloids or alkaloid-like polyamines used in aging control via autophagy modulation are presented in Table 3.
Spermidine, a polyamine rather than a phenolic antioxidant, is generally categorized as a preventative redox modulator [64]. It does not operate as a radical-trapping antioxidant via hydrogen atom transfer. Its biological effects stem from electrostatic interactions with nucleic acids and proteins, modification of acetyl groups, and epigenetic regulation of autophagy genes [65]. Its solubility in water facilitates distribution within the cytosol and nucleus. Spermidine indirectly diminishes ROS via improving mitochondrial quality control and facilitating autophagic clearance, rather than directly neutralizing superoxide, hydroxyl radicals, or nitrogen radicals [66]. It facilitates glutathione homeostasis through enhanced cellular turnover. Berberine, tetrandrine, matrine, harmine, piperine, capsaicin, evodiamine, and galantamine are heterocyclic alkaloids characterized by considerable lipophilicity [67]. They are more accurately classified as preventative antioxidants and redox-modulating signaling agents instead of traditional radical-trapping antioxidants [68]. Their processes entail the control of mitochondrial reactive oxygen species generation, activation of AMPK, and inhibition of mTOR, rather than direct hydrogen atom transfer chemistry [69]. Their radical scavenging ability is constrained relative to polyphenols; however, some can moderately diminish superoxide and nitric oxide concentrations in aqueous settings. The polarity of solvents affects membrane permeability and mitochondrial localization, especially for lipophilic compounds such as capsaicin and piperine [70]. These alkaloids typically contribute to redox homeostasis indirectly by enhancing the expression of endogenous antioxidant enzymes, including superoxide dismutase, catalase, and glutathione peroxidase [71]. Multiple agents augment the restoration of glutathione levels and facilitate redox cycling mechanisms involving coenzyme Q10 and lipoic acid, whereas the protective effects on α-tocopherol are subordinate to membrane stabilization [72].
Table 3.
Alkaloid chemicals that serve as autophagy modulators relevant to human aging biology and longevity regulation.
Terpenoids, including monoterpenes, diterpenes, and triterpenes, are derived from aromatic plants, herbs, and marine organisms [83]. Compounds like ursolic acid, ginsenosides, and andrographolide have been found to modulate autophagy through regulation of mTOR, AMPK, and oxidative stress pathways [84]. Terpenoids often exhibit significant anti-inflammatory properties, which are crucial for maintaining autophagic function in the context of age-related chronic inflammation [85]. Terpenoids indirectly support lysosomal function and autophagic flux by reducing pro-inflammatory cytokine signaling and oxidative damage, thereby promoting tissue homeostasis and longevity [86]. Terpenoids as autophagy modulators essential to human aging biology and longevity regulation, emphasizing AMPK, PI3K/AKT/mTOR, ULK1, TFEB, lysosomal biogenesis, oxidative stress, and inflammation (Table 4).
Terpenoids, including ursolic acid, oleanolic acid, andrographolide, celastrol, carnosic acid, carnosol, dihydroartemisinin, artemisinin, triptolide, ginsenoside Rb1, and ginkgolide B, fundamentally vary from traditional phenolic radical-trapping antioxidants [87]. The majority are more accurately categorized as preventative antioxidants and redox-modulating electrophilic signaling molecules, rather than as direct hydrogen atom-donating antioxidants [88]. Their chemical architectures, characterized by conjugated double bonds, quinone methide groups, lactones, or triterpenoid backbones, promote the regulation of redox-sensitive signaling proteins instead of immediate radical scavenging [89]. Reaction methods generally encompass Michael addition or redox-sensitive cysteine interactions within Keap1, AMPK-regulatory complexes, or other thiol-containing proteins, hence indirectly modulating ROS generation and the expression of antioxidant enzymes [90]. In most triterpenoids, direct sequential proton-loss electron transfer pathways are negligible, unless in the presence of phenolic moieties, as observed in carnosic acid and carnosol, which exhibit traditional hydrogen atom-donating capabilities and lipid radical-trapping qualities [91].
The properties and polarity of solvents significantly affect their biological behavior. Numerous terpenoids exhibit significant lipophilicity, facilitating membrane partitioning and mitochondrial localization [92]. This lipophilicity facilitates the suppression of lipid peroxidation and the stabilization of membrane-associated oxidative processes; however, it constrains aqueous radical scavenging [93]. Instead of directly neutralizing O2•−, •OH, or nitrogen radicals, terpenoids primarily mitigate oxidative stress by stimulating endogenous antioxidant mechanisms, such as superoxide dismutase, catalase, glutathione peroxidase, and Nrf2-regulated enzymes [94]. Various compounds, notably carnosic acid and celastrol, aid in the preservation of glutathione redox equilibrium and indirectly promote the regeneration of α-tocopherol and coenzyme Q10 by sustaining overall cellular reducing capacity [95].
Table 4.
Terpenoids as autophagy modulators related to human aging biology and longevity regulation.
Carotenoids, such as beta-carotene, lycopene, lutein, and astaxanthin, are lipid-soluble pigments found in fruits, vegetables, and marine organisms [106]. While carotenoids are primarily known for their antioxidant properties, they also influence autophagy by modulating redox-sensitive signaling pathways. By preserving redox balance, carotenoids prevent redox-mediated impairment of autophagy-related proteins and lysosomal enzymes. Emerging evidence suggests that carotenoids may also impact AMPK and TFEB activity, promoting mitochondrial turnover and cellular renewal during aging [107]. The most important carotenoids that function as autophagy modulators and are crucial to human aging biology and longevity regulation are presented in Table 5. These compounds influence redox-sensitive signaling pathways, AMPK-mTOR regulation, TFEB-associated lysosomal competence, and the restoration of autophagic flux.
Carotenoids, including β-carotene, lycopene, lutein, zeaxanthin, zeaxanthin dipalmitate, astaxanthin, fucoxanthin, β-cryptoxanthin, canthaxanthin, crocetin, and bixin, are predominantly categorized as lipophilic, chain-breaking radical-trapping antioxidants and physical quenchers of singlet oxygen [108,109]. Their conjugated polyene backbones facilitate electron transfer and radical adduct generation methods, as opposed to the usual sequential proton-loss electron transfer characteristic of phenolics [110]. The donation of hydrogen atoms is of lesser significance compared to energy transfer and radical scavenging stabilized by conjugation.
Their antioxidant activity is significantly influenced by solvent polarity and oxygen tension. Carotenoids have significant lipophilicity and are situated within lipid bilayers, mitochondria, and lipoproteins, where they effectively neutralize lipid peroxyl radicals (ROO•) and quench singlet oxygen [111]. Their activity escalates in hydrophobic membrane settings, while aqueous radical scavenging is constrained [112]. At elevated oxygen levels, several carotenoids may display pro-oxidant properties, underscoring context dependence [113]. They are very efficacious against peroxyl radicals and singlet oxygen, and they indirectly reduce the generation of superoxide and hydroxyl radicals by constraining lipid peroxidation cascades [114]. Direct reactivity with nitric oxide species is constrained, although indirect anti-nitrosative effects arise from the maintenance of membrane integrity.
Carotenoids do not directly facilitate the enzymatic decomposition of ROS/RNS but augment intrinsic defense mechanisms via Nrf2 activation and the maintenance of glutathione reserves [115]. Carotenoids play a crucial role in regenerating α-tocopherol in membranes by diminishing the tocopheroxyl radical [116]. They additionally facilitate redox cycling systems that involve glutathione and coenzyme Q10 by stabilizing lipid compartments [117]. This comprehensive chemical–physiological research elucidates that carotenoids primarily act as membrane-localized radical quenchers and redox stabilizers, with their autophagy-modulating activities intricately associated with the maintenance of lysosomal and mitochondrial integrity during aging [118].
Table 5.
Carotenoids function as autophagy modulators critical to human aging biology and longevity regulation.
Bioactive natural compounds collectively modulate autophagy, reduce oxidative stress, regulate inflammation, and support mitochondrial homeostasis [130]. The ability of these compounds to restore autophagic balance, rather than causing unregulated autophagy induction, is particularly relevant for aging and lifespan control, where fine-tuned regulation is crucial. These compounds mimic aspects of caloric restriction and metabolic adaptation, offering a nutraceutical-based approach to modulating aging pathways. While challenges in bioavailability, dosage optimization, and tissue specificity remain, bioactive natural products hold promise as a foundation for developing safe and effective autophagy-targeted interventions to promote healthy human aging and longevity.
4. Pharmacokinetic and Pharmacodynamic Considerations of Bioactive Natural Compounds Targeting Autophagy and Mitochondrial Health in Aging
An exhaustive assessment of the drugs’ potential utility necessitates the incorporation of pharmacokinetic and pharmacodynamic factors, in conjunction with their redox chemistry and autophagy-modulating characteristics. Despite numerous polyphenols, flavonoids, terpenoids, alkaloids, and carotenoids exhibiting significant mechanistic effects in vitro and in animal models, their translational significance in aging biology is fundamentally contingent upon absorption, bioavailability, tissue distribution, metabolism, excretion, and molecular target interaction.
4.1. Pharmacokinetics
Polyphenols like resveratrol, quercetin, fisetin, and EGCG typically demonstrate moderate oral absorption but display low systemic bioavailability due to swift phase II metabolism, encompassing glucuronidation, sulfation, and methylation [131]. Their circulating forms are frequently conjugated metabolites rather than free aglycones, potentially affecting efficacy and cellular uptake. Lipophilic terpenoids, including ursolic acid, oleanolic acid, celastrol, and ginsenosides, have restricted water solubility and inconsistent intestinal absorption, frequently influenced by dietary lipids, micellar integration, or microbial degradation [132]. Carotenoids such as β-carotene, lycopene, lutein, and astaxanthin are extremely lipophilic and necessitate lipid-rich diets for maximum absorption; they accumulate in membranes, mitochondria, and lipoproteins, facilitating prolonged antioxidant activity while exhibiting sluggish turnover [133]. Alkaloids like berberine and caffeine are rather well absorbed; yet berberine experiences significant first-pass metabolism and displays low plasma concentrations despite its pharmacological effects, possibly due to tissue buildup and microbiome-mediated biotransformation [134]. Spermidine is effectively absorbed and widely disseminated, indicating its intrinsic biological function [135]. Mitochondrial targeting is influenced by distribution patterns. Lipophilic substances preferentially associate with lipid bilayers and mitochondrial membranes, augmenting their capacity to inhibit lipid peroxidation and maintain mitochondrial integrity [136]. Hydrophilic flavonoids may primarily reside in the cytosol unless altered to enhance membrane permeability [137]. Polyphenols are predominantly excreted through renal and biliary routes as conjugates, while carotenoids demonstrate extended half-lives owing to adipose storage [138]. These pharmacokinetic characteristics partially elucidate the discrepancy between in vitro dosage and attainable human plasma concentrations.
4.2. Pharmacodynamics
In addition to direct radical scavenging, most chemicals demonstrate biological effects via receptor-mediated and post-receptor signaling interactions. Polyphenols and flavonoids often activate AMPK, inhibit mTORC1, modify SIRT1, and facilitate TFEB nuclear translocation, hence improving autophagic flux and mitochondrial quality control [139]. Terpenoids like celastrol and carnosic acid may engage with thiol residues in Keap1, thereby activating Nrf2-dependent antioxidant pathways [140]. Berberine directly activates AMPK by modulating mitochondrial complex I, whereas caffeine affects Ca2+-AMPK signaling pathways [141]. Spermidine modifies the state of acetylation of autophagy-related proteins, signifying an epigenetic pharmacodynamic mechanism [65]. Post-receptor effects encompass phosphorylation cascades, modification of redox-sensitive cysteine residues, changes in mitochondrial membrane potential, and regulation of lysosomal activity [142]. Notably, dose-dependent hormetic responses are prevalent; moderate autophagy promotes cellular homeostasis, whereas excessive activation may lead to cytotoxicity.
The pharmacokinetic and pharmacodynamic factors collectively highlight that the ability of bioactive natural substances to modulate autophagy and mitochondria in aging cannot be determined merely by their in vitro antioxidant capability. Therapeutic significance is contingent upon tissue-specific distribution, metabolic transformation, molecular target engagement, and context-dependent signaling integration.
5. Plant-Derived Bioactive Natural Products in Metabolic and Lipid-Modulating Contexts Relevant to Autophagy Modulation in Human Aging
Plant-derived bioactive natural compounds significantly influence the regulation of metabolic and lipid balance; processes intricately associated with autophagy and the biology of aging [143]. Age-related metabolic dysfunction, including insulin resistance, dyslipidemia, visceral fat accumulation, and persistent low-grade inflammation, leads to compromised autophagic flux and expedited cellular senescence [144]. Recent research indicates that certain plant-derived chemicals can restore metabolic equilibrium while concurrently regulating autophagy-related signaling pathways. Polyphenols, including resveratrol, quercetin, and epigallocatechin gallate, stimulate AMPK and SIRT1 signaling while inhibiting mTORC1 activity, thus augmenting autophagic flux and boosting mitochondrial quality control [145]. Curcumin and berberine exhibit lipid-lowering effects by modulating hepatic lipid metabolism, enhancing insulin sensitivity, and reducing oxidative stress, mechanisms often associated with increased LC3-II formation and decreased p62 accumulation in experimental models [146]. Carotenoids, such as lycopene and astaxanthin, enhance redox stability and safeguard against lipid peroxidation, thereby indirectly bolstering lysosomal functionality and autophagy efficacy [147]. In human observational and interventional studies, plant-derived extracts have demonstrated enhancements in lipid profiles, inflammatory markers, and metabolic parameters related to aging [148]. Nevertheless, direct assessment of autophagy in humans is constrained, with most conclusions derived from subsequent metabolic results. These bioactive chemicals collectively serve as potential modulators of the metabolic-autophagy axis in human aging; nevertheless, long-term, biomarker-guided clinical investigations are necessary to validate their effects on lifespan.
6. Preclinical Findings and Human Observational or Interventional Evidence of Bioactive Natural Products in Autophagy Modulation During Human Aging
Preclinical research furnishes substantial mechanistic evidence that several bioactive natural compounds influence autophagy pathways pertinent to aging biology. In cellular and animal models, compounds such as spermidine, resveratrol, curcumin, quercetin, and epigallocatechin gallate activate AMPK, inhibit mTORC1, enhance SIRT1 signaling, and promote TFEB-mediated lysosomal biogenesis, collectively restoring autophagic flux and improving mitochondrial quality control [139,149]. These therapies often enhance metabolic balance, diminish oxidative stress, mitigate inflammation, and prolong lifespan in model species. Conversely, human evidence is still relatively scarce but is developing. Observational cohort studies indicate correlations between increased consumption of polyphenol-rich or spermidine-rich foods and decreased all-cause mortality, enhanced cardiovascular health, and reduced inflammatory burden [150]. Small-scale interventional trials have demonstrated that spermidine supplementation can enhance indicators of cognitive function and cellular aging, whereas resveratrol and polyphenol-based therapies influence metabolic parameters and inflammatory markers, aligning with autophagy-related pathways [151]. Nonetheless, direct quantification of autophagic flux in humans continues to pose significant technical challenges, leading most investigations to depend on indirect indicators [152]. These findings collectively underscore promising translational significance while emphasizing the necessity for rigorously controlled longitudinal studies to ascertain causal impacts on human lifespan.
7. Therapeutic and Clinical Application of Bioactive Natural Products Autophagy Modulation in Aging
Translation of autophagy-modulating natural products into the clinic is now moving from mechanistic rationalization to measurable human phenotypes, but it has been uneven. The most “clinically mature” cases are where the therapies enhance mitochondrial quality control or restore autophagic function in aging-related tissues such as skeletal muscle, immune cells, and metabolic organs. One well-studied example is urolithin A, a gut-produced postbiotic from ellagitannin-rich foods like pomegranate. Human studies have shown that it is safe and can produce a molecular profile that is consistent with improved mitochondrial and cellular health commensurate with its role as a mitophagy inducer. This provides a relatively pragmatic translational approach: use a well-characterized compound, target a defined aging phenotype (mitophagy), and then measure functional readouts (strength, endurance) with molecular biomarkers (Figure 4).
Figure 4.
Translational pathway of bioactive natural products in autophagy and mitophagy regulation during aging. Natural product consumption emphasizes key sources such as pomegranate (precursors of urolithin A), wheat germ and cereal grains (spermidine), grapes (resveratrol), and turmeric (curcumin). Metabolism highlights the essential function of gut microbiota in transforming food precursors into bioactive metabolites, especially postbiotic molecules like urolithin A. Target tissues encompass metabolically active and aging-sensitive systems, including skeletal muscle, immunological cells (particularly T cells), and the liver, where a loss in autophagy contributes to functional degradation. Cellular mechanisms illustrate the activation of AMPK and SIRT1 signaling, along with the inhibition of mTOR, resulting in the induction of autophagy and selective mitophagy, autophagosome formation, and autolysosomal destruction of impaired mitochondria. The lower panels encapsulate essential translational examples: (A) Urolithin A promotes mitophagy, augments PGC-1α signaling, diminishes oxidative stress, and enhances muscle endurance in a dose- and time-dependent fashion. (B) Spermidine facilitates fasting-induced autophagy and maintains autophagic efficacy in aging T cells. (C) Polyphenols, including resveratrol and curcumin, influence AMPK-SIRT1-mTOR signaling to regulate autophagy, thereby contributing to cardiometabolic protection and the attenuation of inflammation.
Clinical studies often use surrogate outcomes like inflammation or metabolic markers, while direct measurement of autophagic flux in humans is limited by the lack of standardized, non-invasive biomarkers. Natural products are chemically heterogeneous and can vary between preparations, posing reproducibility and standardization challenges. Aging is highly heterogeneous between individuals, and comorbidities, polypharmacy, and sex-specific factors can confound interpretation and limit generalizability.
Another clinically relevant axis is spermidine, a supplemental autophagy inducer that declines in human T cells with age. A long-term randomized trial in older individuals at risk of Alzheimer’s disease did not improve memory but did provide clarity on feasibility and biomarker approaches for future studies. Spermidine is mechanistically linked to fasting-mediated autophagy, and the data from human subjects is consistent with an in vivo role. The clinical use of more traditional polyphenols like resveratrol and curcumin has been focused on cardiometabolic and inflammatory endpoints, but direct autophagy-flux biomarkers in humans are rare. The strongest data set here remains at the molecular and preclinical level with respect to AMPK, SIRT1, and mTOR-related autophagy regulation. Current uses are moving towards using standardizable biomarkers, dose refinement, and formulations with better bioavailability and tissue targeting. Table 6 presents clinical and translational examples of natural compounds that influence autophagy or mitophagy in the context of aging.
Table 6.
Therapeutic and clinical applications of bioactive natural products in the control of autophagy related to aging.
8. Translational Limitations of Bioactive Natural Products Targeting Autophagy in Human Aging
Despite strong mechanistic evidence from cellular and animal models, substantial translational obstacles hinder the therapeutic use of bioactive natural compounds as autophagy modulators in human aging. Bioavailability is a big problem. A lot of polyphenols and related compounds, such as resveratrol and curcumin, do not dissolve well, break down quickly, or get into the body very easily, which makes it hard to get concentrations that are like those employed in experimental settings [159]. The amount of the drug is still a big problem. In vitro, effective concentrations are often beyond levels attainable by diet alone, and consistent dosage regimens in humans are not yet well established. Moreover, the long-term safety profile of persistent autophagy regulation is not yet fully understood. Moderate activation of autophagy may facilitate cellular homeostasis; however, excessive or prolonged activation could potentially lead to muscular atrophy, disrupted immunological equilibrium, or unexpected metabolic consequences, especially in older adults [160]. Another significant factor is inter-individual variability. Genetic background, epigenetic status, gut microbiome makeup, nutritional condition, comorbidities, and sex-specific variations all affect how well autophagy works [161]. Aging modifies pharmacokinetics and stress signaling pathways, challenging the extrapolation from controlled models to diverse human populations. To overcome these translational challenges, we will need standardized formulations, dosage regimens based on biomarkers, and well-planned, long-term clinical trials that target different groups of older people.
9. Limitations and Future Direction of Bioactive Natural Products in Autophagy Modulation in Aging
There are multiple limitations in translating the strong molecular relationships between bioactive natural products and autophagy regulation to clinical aging. Drugs have poor oral bioavailability, rapid metabolism, and inter-individual variability related to alterations in gut microbiota, which can lead to inconsistent tissue exposure and variable responses. Autophagy is highly context-dependent and too much or too little autophagy can be detrimental, and as such, the dosage, timing, and tissue specificity of these interventions are key, but are often not well-defined.
For future progress, robust translation strategies will be needed to bridge autophagy modulation and quantifiable clinical endpoints. The development of standardized biomarkers for human autophagy and lysosomal function, including blood-based signatures, imaging modalities, and validated surrogate markers will help improve the interpretability of studies. Improved formulations, including nanoparticle delivery systems, prodrugs, and microbiome-informed postbiotics, could improve bioavailability and allow for tissue-specific targeting while reducing off-target effects. Personalized approaches will be needed to stratify subjects based on metabolic state, inflammatory burden, microbiome composition, and genetic variability in autophagy pathways to identify responders and optimize dosing regimens. Synergistic interventions that combine natural products with lifestyle interventions like exercise, time-restricted feeding, or protein periodization may produce additive effects on AMPK, SIRT1, TFEB, and mitophagy pathways relevant to healthy aging. In the long term, large-scale randomized controlled trials with standardized endpoints and long-term safety evaluations will be essential to move autophagy-targeting natural products from promising candidates to evidence-based interventions for aging.
10. Conclusions
Autophagy is a pivotal regulatory process that connects cellular quality control with aging and longevity, and its gradual decline considerably contributes to age-related functional decline and disease vulnerability. Increasing data indicates that bioactive natural compounds, including polyphenols, flavonoids, alkaloids, terpenoids, and carotenoids, can regulate autophagy in a nuanced and context-sensitive manner. Instead of serving as indiscriminate autophagy inducers, these drugs precisely modulate critical signaling pathways, including AMPK, PI3K/AKT/mTOR, SIRT1, FOXO, and TFEB, while concurrently diminishing oxidative stress and chronic inflammation that hinder autophagic flux in aging. These coordinated effects enable natural products to promote proteostasis, mitochondrial quality control, and metabolic flexibility, which are crucial for sustaining tissue homeostasis and promoting healthy longevity. Despite ongoing obstacles concerning bioavailability, inter-individual variability, and the validation of clinical biomarkers, advancements in formulation, precision nutrition, and trial design are swiftly enhancing translational potential. Autophagy-targeting bioactive natural compounds collectively constitute a promising, mechanistically sound approach for enhancing healthy human aging and prolonging health span.
Author Contributions
M.J. and M.A.R. writing—original draft, preparing figures, editing and modifying draft preparation. A.H.H. and M.A.-Z. editing—writing, visualization and reviewing. All authors have read and agreed to the published version of the manuscript.
Funding
This work was supported and funded by the Deanship of Scientific Research at Imam Mohammad Ibn Saud Islamic University (IMSIU) (grant number IMSIU-DDRSP2601).
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
No new data were created or analyzed in this study.
Conflicts of Interest
The authors declare no conflict of interest.
References
- Chun, Y.; Kim, J. Autophagy: An Essential Degradation Program for Cellular Homeostasis and Life. Cells 2018, 7, 278. [Google Scholar] [CrossRef] [Scilit]
- Sanada, F.; Hayashi, S.; Morishita, R. Targeting the hallmarks of aging: Mechanisms and therapeutic opportunities. Front. Cardiovasc. Med. 2025, 12, 1631578. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kaarniranta, K.; Uusitalo, H.; Blasiak, J.; Felszeghy, S.; Kannan, R.; Kauppinen, A.; Salminen, A.; Sinha, D.; Ferrington, D. Mechanisms of mitochondrial dysfunction and their impact on age-related macular degeneration. Prog. Retin. Eye Res. 2020, 79, 100858. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Barbosa, M.C.; Grosso, R.A.; Fader, C.M. Hallmarks of Aging: An Autophagic Perspective. Front. Endocrinol. 2018, 9, 790. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Palmer, J.E.; Wilson, N.; Son, S.M.; Obrocki, P.; Wrobel, L.; Rob, M.; Takla, M.; Korolchuk, V.I.; Rubinsztein, D.C. Autophagy, aging, and age-related neurodegeneration. Neuron 2025, 113, 29–48. [Google Scholar] [CrossRef] [Scilit]
- Nieto-Torres, J.L.; Hansen, M. Macroautophagy and aging: The impact of cellular recycling on health and longevity. Mol. Asp. Med. 2021, 82, 101020. [Google Scholar] [CrossRef] [Scilit]
- Rahman, M.A.; Rakib-Uz-Zaman, S.M.; Chakraborti, S.; Bhajan, S.K.; Gupta, R.D.; Jalouli, M.; Parvez, M.A.K.; Shaikh, M.H.; Hoque Apu, E.; Harrath, A.H.; et al. Advancements in Utilizing Natural Compounds for Modulating Autophagy in Liver Cancer: Molecular Mechanisms and Therapeutic Targets. Cells 2024, 13, 1186. [Google Scholar] [CrossRef] [Scilit]
- Stacchiotti, A.; Corsetti, G. Natural Compounds and Autophagy: Allies Against Neurodegeneration. Front. Cell Dev. Biol. 2020, 8, 555409. [Google Scholar] [CrossRef] [Scilit]
- Ponce-Mora, A.; Salazar, N.A.; Domenech-Bendaña, A.; Locascio, A.; Bejarano, E.; Gimeno-Mallench, L. Interplay Between Polyphenols and Autophagy: Insights From an Aging Perspective. Front. Biosci. 2025, 30, 25728. [Google Scholar] [CrossRef] [Scilit]
- Liu, F.; Zhao, L.; Wu, T.; Yu, W.; Li, J.; Wang, W.; Huang, C.; Diao, Z.; Xu, Y. Targeting autophagy with natural products as a potential therapeutic approach for diabetic microangiopathy. Front. Pharmacol. 2024, 15, 1364616. [Google Scholar] [CrossRef] [Scilit]
- Rahman, M.A.; Jalouli, M.; Al-Zharani, M.; Hoque Apu, E.; Harrath, A.H. Mechanistic Insights into Autophagy-Dependent Cell Death (ADCD): A Novel Avenue for Cancer Therapy. Cells 2025, 14, 1072. [Google Scholar] [CrossRef] [Scilit]
- Jeong, S.Y. The Role of Mammalian Target of Rapamycin (mTOR) and Adenosine Monophosphate-Activated Protein Kinase (AMPK) Signaling in Skeletal Muscle Hypertrophy: A Literature Review with Implications for Health and Disease. Cureus 2025, 17, e96018. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mandic, M.; Misirkic Marjanovic, M.; Janjetovic, K.; Bosnjak, M.; Harhaji-Trajkovic, L.; Trajkovic, V.; Vucicevic, L. Multifaceted Role AMPK Autophagy: More Than A Simple Trigger? Am. J. Physiol. Cell Physiol. 2025, 329, C1380–C1397. [Google Scholar] [CrossRef] [Scilit]
- Rahman, M.A.; Shaikh, M.H.; Gupta, R.D.; Siddika, N.; Shaikh, M.S.; Zafar, M.S.; Kim, B.; Hoque Apu, E. Advancements in autophagy modulation for the management of oral disease: A focus on drug targets and therapeutics. Biomedicines 2024, 12, 2645. [Google Scholar] [CrossRef] [Scilit]
- Ding, X.; Zhu, C.; Wang, W.; Li, M.; Ma, C.; Gao, B. SIRT1 is a regulator of autophagy: Implications for the progression and treatment of myocardial ischemia-reperfusion. Pharmacol. Res. 2024, 199, 106957. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Son, Y.; Han, M.; Wu, X.; Roh, Y.S. SIRT1-Mediated Redox and Senescence Regulation in Cancer: Mechanisms and Therapeutic Implications. Antioxidants 2025, 14, 1076. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Franco-Juárez, B.; Coronel-Cruz, C.; Hernández-Ochoa, B.; Gómez-Manzo, S.; Cárdenas-Rodríguez, N.; Arreguin-Espinosa, R.; Bandala, C.; Canseco-Ávila, L.M.; Ortega-Cuellar, D. TFEB; Beyond Its Role Autophagy Lysosomes Regulator. Cells 2022, 11, 3153. [Google Scholar] [CrossRef] [Scilit]
- Bala, S.; Szabo, G. TFEB, a master regulator of lysosome biogenesis and autophagy, is a new player in alcoholic liver disease. Dig. Med. Res. 2018, 1, 3153. [Google Scholar] [CrossRef] [Scilit]
- Mundo Rivera, V.M.; Tlacuahuac Juárez, J.R.; Murillo Melo, N.M.; Leyva Garcia, N.; Magaña, J.J.; Cordero Martínez, J.; Jiménez Gutierrez, G.E. Natural Autophagy Activators to Fight Age-Related Diseases. Cells 2024, 13, 1611. [Google Scholar] [CrossRef] [Scilit]
- Jia, J.; Bissa, B.; Brecht, L.; Allers, L.; Choi, S.W.; Gu, Y.; Zbinden, M.; Burge, M.R.; Timmins, G.; Hallows, K.; et al. AMPK, a Regulator of Metabolism and Autophagy, Is Activated by Lysosomal Damage via a Novel Galectin-Directed Ubiquitin Signal Transduction System. Mol. Cell 2020, 77, 951–969.e9. [Google Scholar] [CrossRef] [Scilit]
- Rudrapal, M.; Khairnar, S.J.; Khan, J.; Dukhyil, A.B.; Ansari, M.A.; Alomary, M.N.; Alshabrmi, F.M.; Palai, S.; Deb, P.K.; Devi, R. Dietary Polyphenols and Their Role in Oxidative Stress-Induced Human Diseases: Insights into Protective Effects, Antioxidant Potentials and Mechanism(s) of Action. Front. Pharmacol. 2022, 13, 806470. [Google Scholar] [CrossRef] [Scilit]
- De Sousa, R. Molecular crosstalk for longevity: Exercise and the AMPK/SIRT1/PGC-1α/Irisin/BDNF axis. Mol. Biol. Rep. 2025, 53, 142. [Google Scholar] [CrossRef] [Scilit]
- Leri, M.; Scuto, M.; Ontario, M.L.; Calabrese, V.; Calabrese, E.J.; Bucciantini, M.; Stefani, M. Healthy Effects of Plant Polyphenols: Molecular Mechanisms. Int. J. Mol. Sci. 2020, 21, 1250. [Google Scholar] [CrossRef] [Scilit]
- Salehi, B.; Mishra, A.P.; Nigam, M.; Sener, B.; Kilic, M.; Sharifi-Rad, M.; Fokou, P.V.T.; Martins, N.; Sharifi-Rad, J. Resveratrol: A double-edged sword in health benefits. Biomedicines 2018, 6, 91. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Khosravi, A.; Deyhim, M.R.; Yari, F.; Zarif, M.N. Resveratrol; a Double-Edged Sword Antioxidant Agent for Preserving Platelet Cell Functions During Storage; Molecular Insights. Rep. Biochem. Mol. Biol. 2023, 11, 553. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Heurtaux, T.; Bouvier, D.S.; Benani, A.; Helgueta Romero, S.; Frauenknecht, K.B.; Mittelbronn, M.; Sinkkonen, L. Normal and pathological NRF2 signalling in the central nervous system. Antioxidants 2022, 11, 1426. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lee, W.-H.; Loo, C.-Y.; Bebawy, M.; Luk, F.; Mason, R.S.; Rohanizadeh, R. Curcumin and its derivatives: Their application in neuropharmacology and neuroscience in the 21st century. Curr. Neuropharmacol. 2013, 11, 338–378. [Google Scholar] [CrossRef] [Scilit]
- Cheng, M.; Ding, F.; Li, L.; Dai, C.; Sun, X.; Xu, J.; Chen, F.; Li, M.; Li, X. Exploring the role of curcumin in mitigating oxidative stress to alleviate lipid metabolism disorders. Front. Pharmacol. 2025, 16, 1517174. [Google Scholar] [CrossRef] [Scilit]
- Kumar, N.; Goel, N. Phenolic acids: Natural versatile molecules with promising therapeutic applications. Biotechnol. Rep. 2019, 24, e00370. [Google Scholar] [CrossRef] [Scilit]
- Kalu, A.; Ray, S.K. Epigallocatechin-3-Gallate, quercetin, and Kaempferol for treatment of Parkinson’s disease through prevention of gut Dysbiosis and attenuation of multiple molecular mechanisms of pathogenesis. Brain Sci. 2025, 15, 144. [Google Scholar] [CrossRef] [Scilit]
- Kagan, V.E.; Straub, A.C.; Tyurina, Y.Y.; Kapralov, A.A.; Hall, R.; Wenzel, S.E.; Mallampalli, R.K.; Bayir, H. Vitamin E/coenzyme Q-dependent “free radical reductases”: Redox regulators in ferroptosis. Antioxid. Redox Signal. 2024, 40, 317–328. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Rogina, B.; Tissenbaum, H.A. SIRT1, resveratrol and aging. Front. Genet. 2024, 15, 1393181. [Google Scholar] [CrossRef] [Scilit]
- Ahmed, M. Targeting aging pathways with natural compounds: A review of curcumin, epigallocatechin gallate, thymoquinone, and resveratrol. Immun. Ageing 2025, 22, 28. [Google Scholar] [CrossRef] [Scilit]
- Holczer, M.; Besze, B.; Zámbó, V.; Csala, M.; Bánhegyi, G.; Kapuy, O. Epigallocatechin-3-Gallate (EGCG) Promotes Autophagy-Dependent Survival via Influencing the Balance of mTOR-AMPK Pathways upon Endoplasmic Reticulum Stress. Oxidative Med. Cell. Longev. 2018, 2018, 6721530. [Google Scholar] [CrossRef] [Scilit]
- Jin, T.; Zhang, Y.; Botchway, B.O.; Huang, M.; Lu, Q.; Liu, X. Quercetin activates the Sestrin2/AMPK/SIRT1 axis to improve amyotrophic lateral sclerosis. Biomed. Pharmacother. 2023, 161, 114515. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Suh, Y.; Afaq, F.; Khan, N.; Johnson, J.J.; Khusro, F.H.; Mukhtar, H. Fisetin induces autophagic cell death through suppression of mTOR signaling pathway in prostate cancer cells. Carcinogenesis 2010, 31, 1424–1433. [Google Scholar] [CrossRef] [Scilit]
- Han, B.; Yu, Y.-Q.; Yang, Q.-L.; Shen, C.-Y.; Wang, X.-J. Kaempferol induces autophagic cell death of hepatocellular carcinoma cells via activating AMPK signaling. Oncotarget 2017, 8, 86227. [Google Scholar] [CrossRef] [Scilit]
- Tong, X.; Smith, K.A.; Pelling, J.C. Apigenin, a chemopreventive bioflavonoid, induces AMP-activated protein kinase activation in human keratinocytes. Mol. Carcinog. 2012, 51, 268–279. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tang, L.; Fan, X.; Xu, Y.; Zhang, Y.; Li, G. Luteolin Inhibits Dexamethasone-Induced Osteoporosis by Autophagy Activation Through miR-125b-5p/SIRT3/AMPK/mTOR Axis, an In Vitro and In Vivo Study. Food Sci. Nutr. 2025, 13, e70071. [Google Scholar] [CrossRef] [Scilit]
- Pierzynowska, K.; Podlacha, M.; Gaffke, L.; Majkutewicz, I.; Mantej, J.; Węgrzyn, A.; Osiadły, M.; Myślińska, D.; Węgrzyn, G. Autophagy-dependent mechanism of genistein-mediated elimination of behavioral and biochemical defects in the rat model of sporadic Alzheimer’s disease. Neuropharmacology 2019, 148, 332–346. [Google Scholar] [CrossRef] [Scilit]
- Yao, Y.-X.; Yao, C.-H.; Zhang, C.-Y.; Peng, X.-Z.; Dai, S.; Yu, Y.-J.; Li, Y.-Z.; Zhang, S.-L.; Li, Y.-X. Chlorogenic Acid Ameliorates Acetaminophen-Induced Liver Injury Through AMPK/mTOR/ULK1-Mediated Autophagy Activation. Am. J. Chin. Med. 2025, 53, 523–542. [Google Scholar] [CrossRef] [Scilit]
- Kumar, S.; Pandey, A.K. Chemistry and biological activities of flavonoids: An overview. Sci. World J. 2013, 2013, 162750. [Google Scholar] [CrossRef] [Scilit]
- Pang, X.; Zhang, X.; Jiang, Y.; Su, Q.; Li, Q.; Li, Z. Autophagy: Mechanisms and Therapeutic Potential of Flavonoids in Cancer. Biomolecules 2021, 11, 135. [Google Scholar] [CrossRef] [Scilit]
- Zughaibi, T.A.; Suhail, M.; Tarique, M.; Tabrez, S. Targeting PI3K/Akt/mTOR Pathway by Different Flavonoids: A Cancer Chemopreventive Approach. Int. J. Mol. Sci. 2021, 22, 12455. [Google Scholar] [CrossRef] [Scilit]
- Miean, K.H.; Mohamed, S. Flavonoid (myricetin, quercetin, kaempferol, luteolin, and apigenin) content of edible tropical plants. J. Agric. Food Chem. 2001, 49, 3106–3112. [Google Scholar] [CrossRef] [Scilit]
- Chen, B.; Su, J.; Hu, Y.; Liu, S.; Ouyang, X.; Cai, R.; You, X.; Li, X. Antioxidant mechanisms and products of four 4′, 5, 7-trihydroxyflavonoids with different structural types. RSC Med. Chem. 2023, 14, 173–182. [Google Scholar] [CrossRef] [Scilit]
- Bouaziz, A. Screening of the Antioxidant and Hypotensive Activities of Some Medicinal Plants in Relation to Their Polyphenolic Contents. Ph.D. Thesis, Université Ferhat Abbas, Sétif, Algeria, 2018. [Google Scholar]
- Miličević, A. Flavonoid oxidation potentials and antioxidant activities-theoretical models based on oxidation mechanisms and related changes in electronic structure. Int. J. Mol. Sci. 2024, 25, 5011. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Teng, H.; Zheng, Y.; Cao, H.; Huang, Q.; Xiao, J.; Chen, L. Enhancement of bioavailability and bioactivity of diet-derived flavonoids by application of nanotechnology: A review. Crit. Rev. Food Sci. Nutr. 2023, 63, 378–393. [Google Scholar] [CrossRef] [Scilit]
- Nacaia, H.; Takekoshi, S.; Takagi, T.; Honma, T.; Watanabe, K. Antioxidative action of flavonoids quercetin and catechin, mediated by the activation of glutathione peroxidase. Tokai J. Exp. Clin. Med. 1999, 24, 1–11. [Google Scholar]
- Rodella, U.; Honisch, C.; Gatto, C.; Ruzza, P.; D’Amato Tóthová, J. Antioxidant nutraceutical strategies in the prevention of oxidative stress related eye diseases. Nutrients 2023, 15, 2283. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kim, T.W.; Lee, H.G. Apigenin induces autophagy and cell death by targeting EZH2 under hypoxia conditions in gastric cancer cells. Int. J. Mol. Sci. 2021, 22, 13455. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhu, M.-l.; Zhang, P.-m.; Jiang, M.; Yu, S.-w.; Wang, L. Myricetin induces apoptosis and autophagy by inhibiting PI3K/Akt/mTOR signalling in human colon cancer cells. BMC Complement. Med. Ther. 2020, 20, 209. [Google Scholar] [CrossRef] [Scilit]
- Kim, S.; Choi, K.J.; Cho, S.-J.; Yun, S.-M.; Jeon, J.-P.; Koh, Y.H.; Song, J.; Johnson, G.V.; Jo, C. Fisetin stimulates autophagic degradation of phosphorylated tau via the activation of TFEB and Nrf2 transcription factors. Sci. Rep. 2016, 6, 24933. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Huang, Y.; Chen, Y.; Shaw, A.M.; Goldfine, H.; Tian, J.; Cai, J. Enhancing TFEB-mediated cellular degradation pathways by the mTORC1 inhibitor quercetin. Oxidative Med. Cell. Longev. 2018, 2018, 5073420. [Google Scholar] [CrossRef] [Scilit]
- Wang, K.-Y.; Huang, C.-X.; Hu, X.-J.; Liu, J.-Y.; Qin, X.-H.; Tong, C.-X.; Liu, Z.-Q.; He, W.; Jiang, T.-M.; Song, J.-L. Naringenin Alleviates the Autophagy-Associated AMPK-Akt/mTOR Pathway to Regulate Inflammation and Barrier Function, Decreasing DSS-Induced Intestinal Fibrosis. ACS Omega 2025, 10, 40981–40994. [Google Scholar] [CrossRef] [Scilit]
- Saiprasad, G.; Chitra, P.; Manikandan, R.; Sudhandiran, G. Hesperidin induces apoptosis and triggers autophagic markers through inhibition of Aurora-A mediated phosphoinositide-3-kinase/Akt/mammalian target of rapamycin and glycogen synthase kinase-3 beta signalling cascades in experimental colon carcinogenesis. Eur. J. Cancer 2014, 50, 2489–2507. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, M.; Peng, L.; Gong, P.; Zheng, X.; Sun, T.; Zhang, X.; Huo, J. Baicalein induces mitochondrial autophagy to prevent Parkinson’s disease in rats via miR-30b and the SIRT1/AMPK/mTOR pathway. Front. Neurol. 2022, 12, 646817. [Google Scholar] [CrossRef] [Scilit]
- Peng, J.; Zheng, T.T.; Li, X.; Liang, Y.; Wang, L.J.; Huang, Y.C.; Xiao, H.T. Plant-Derived Alkaloids: The Promising Disease-Modifying Agents for Inflammatory Bowel Disease. Front. Pharmacol. 2019, 10, 351. [Google Scholar] [CrossRef] [Scilit]
- Mokhfi, F.Z.; Al Amin, M.; Zehravi, M.; Sweilam, S.H.; Arjun, U.; Gupta, J.K.; Vallamkonda, B.; Balakrishnan, A.; Challa, M.; Singh, J.; et al. Alkaloid-based modulators of the PI3K/Akt/mTOR pathway for cancer therapy: Understandings from pharmacological point of view. Chem. Biol. Interact. 2024, 402, 111218. [Google Scholar] [CrossRef] [Scilit]
- Law, B.Y.; Chan, W.K.; Xu, S.W.; Wang, J.R.; Bai, L.P.; Liu, L.; Wong, V.K. Natural small-molecule enhancers of autophagy induce autophagic cell death in apoptosis-defective cells. Sci. Rep. 2014, 4, 5510. [Google Scholar] [CrossRef] [Scilit]
- Satarker, S.; Wilson, J.; Kolathur, K.K.; Mudgal, J.; Lewis, S.A.; Arora, D.; Nampoothiri, M. Spermidine as an epigenetic regulator of autophagy in neurodegenerative disorders. Eur. J. Pharmacol. 2024, 979, 176823. [Google Scholar] [CrossRef] [Scilit]
- Alshahrani, S.M.; Al-Kuraishy, H.M.; Al-Gareeb, A.I.; Albuhadily, A.K.; Fawzy, M.N.; Kadasah, S.F.; Alruwaili, M.; Papadakis, M.; Alexiou, A.; El-Saber Batiha, G. Berberine’s paradox in Neurodegeneration: Therapeutic promise and safety challenges in Parkinson’s disease. Neuropharmacology 2025, 278, 110555. [Google Scholar] [CrossRef] [Scilit]
- Madeo, F.; Eisenberg, T.; Pietrocola, F.; Kroemer, G. Spermidine in health and disease. Science 2018, 359, eaan2788. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hofer, S.J.; Simon, A.K.; Bergmann, M.; Eisenberg, T.; Kroemer, G.; Madeo, F. Mechanisms of spermidine-induced autophagy and geroprotection. Nat. Aging 2022, 2, 1112–1129. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, R.; Li, X.; Ma, H.; Yang, Q.; Shang, Q.; Song, L.; Zheng, Z.; Zhang, S.; Pan, Y.; Huang, P. Spermidine endows macrophages anti-inflammatory properties by inducing mitochondrial superoxide-dependent AMPK activation, Hif-1α upregulation and autophagy. Free Radic. Biol. Med. 2020, 161, 339–350. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gutiérrez-Grijalva, E.P.; López-Martínez, L.X.; Contreras-Angulo, L.A.; Elizalde-Romero, C.A.; Heredia, J.B. Plant alkaloids: Structures and bioactive properties. In Plant-Derived Bioactives: Chemistry and Mode of Action; Springer: Berlin/Heidelberg, Germany, 2020; pp. 85–117. [Google Scholar]
- Dutta, N.; Pemmaraju, D.B.; Ghosh, S.; Ali, A.; Mondal, A.; Majumder, C.; Nelson, V.K.; Mandal, S.C.; Misra, A.K.; Rengan, A.K. Alkaloid-rich fraction of Ervatamia coronaria sensitizes colorectal cancer through modulating AMPK and mTOR signalling pathways. J. Ethnopharmacol. 2022, 283, 114666. [Google Scholar] [CrossRef] [Scilit]
- Nelson, V.K.; Nuli, M.V.; Mastanaiah, J.; Saleem TS, M.; Birudala, G.; Jamous, Y.F.; Alshargi, O.; Kotha, K.K.; Sudhan, H.H.; Mani, R.R. Reactive oxygen species mediated apoptotic death of colon cancer cells: Therapeutic potential of plant derived alkaloids. Front. Endocrinol. 2023, 14, 1201198. [Google Scholar] [CrossRef] [Scilit]
- Gorgani, L.; Mohammadi, M.; Najafpour, G.D.; Nikzad, M. Piperine—The bioactive compound of black pepper: From isolation to medicinal formulations. Compr. Rev. Food Sci. Food Saf. 2017, 16, 124–140. [Google Scholar] [CrossRef] [Scilit]
- Misra, N.; Gupta, A.K. Effect of salinity and different nitrogen sources on the activity of antioxidant enzymes and indole alkaloid content in Catharanthus roseus seedlings. J. Plant Physiol. 2006, 163, 11–18. [Google Scholar] [CrossRef] [Scilit]
- Sharma, S.; Advani, D.; Das, A.; Malhotra, N.; Khosla, A.; Arora, V.; Jha, A.; Yadav, M.; Ambasta, R.K.; Kumar, P. Pharmacological intervention in oxidative stress as a therapeutic target in neurological disorders. J. Pharm. Pharmacol. 2022, 74, 461–484. [Google Scholar] [CrossRef] [Scilit]
- Pietrocola, F.; Lachkar, S.; Enot, D.P.; Niso-Santano, M.; Bravo-San Pedro, J.M.; Sica, V.; Izzo, V.; Maiuri, M.C.; Madeo, F.; Mariño, G. Spermidine induces autophagy by inhibiting the acetyltransferase EP300. Cell Death Differ. 2015, 22, 509–516. [Google Scholar] [CrossRef] [Scilit]
- Xu, Z.; Feng, W.; Shen, Q.; Yu, N.; Yu, K.; Wang, S.; Chen, Z.; Shioda, S.; Guo, Y. Rhizoma coptidis and berberine as a natural drug to combat aging and aging-related diseases via anti-oxidation and AMPK activation. Aging Dis. 2017, 8, 760. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pietrocola, F.; Malik, S.A.; Mariño, G.; Vacchelli, E.; Senovilla, L.; Chaba, K.; Niso-Santano, M.; Maiuri, M.C.; Madeo, F.; Kroemer, G. Coffee induces autophagy in vivo. Cell Cycle 2014, 13, 1987–1994. [Google Scholar] [CrossRef] [Scilit]
- Wong, V.K.W.; Zeng, W.; Chen, J.; Yao, X.J.; Leung, E.L.H.; Wang, Q.Q.; Chiu, P.; Ko, B.C.; Law, B.Y.K. Tetrandrine, an activator of autophagy, induces autophagic cell death via PKC-α inhibition and mTOR-dependent mechanisms. Front. Pharmacol. 2017, 8, 351. [Google Scholar] [CrossRef] [Scilit]
- Li, X.; Zhou, J.; Ling, Y.; Tan, Y.; Zhang, J.; Wang, X.; Li, F.; Jiang, S.; Zhang, S.; Yu, K. Matrine induces autophagic cell death by triggering ROS/AMPK/mTOR axis and apoptosis in multiple myeloma. Biomed. Pharmacother. 2024, 175, 116738. [Google Scholar] [CrossRef] [Scilit]
- Hu, Y.; Yu, X.; Yang, L.; Xue, G.; Wei, Q.; Han, Z.; Chen, H. Research progress on the antitumor effects of harmine. Front. Oncol. 2024, 14, 1382142. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, J.; Chen, M.; Wang, X.; Wang, Y.; Duan, C.; Gao, G.; Lu, L.; Wu, X.; Wang, X.; Yang, H. Piperine induces autophagy by enhancing protein phosphotase 2A activity in a rotenone-induced Parkinson’s disease model. Oncotarget 2016, 7, 60823. [Google Scholar] [CrossRef] [Scilit]
- Que, T.; Ren, B.; Fan, Y.; Liu, T.; Hou, T.; Dan, W.; Liu, B.; Wei, Y.; Lei, Y.; Zeng, J. Capsaicin inhibits the migration, invasion and EMT of renal cancer cells by inducing AMPK/mTOR-mediated autophagy. Chem. Biol. Interact. 2022, 366, 110043. [Google Scholar] [CrossRef] [Scilit]
- Li, B.; Liu, J.; Zhang, D.; Chu, Y.; Chen, Z.; Tsao, J.; Chen, T.; Jiang, J.; Hu, K. Evodiamine promotes autophagy and alleviates oxidative stress in dry eye disease through the p53/mTOR pathway. Investig. Ophthalmol. Vis. Sci. 2025, 66, 44. [Google Scholar] [CrossRef] [Scilit]
- Jiang, S.; Zhao, Y.; Zhang, T.; Lan, J.; Yang, J.; Yuan, L.; Zhang, Q.; Pan, K.; Zhang, K. Galantamine inhibits β-amyloid-induced cytostatic autophagy in PC 12 cells through decreasing ROS production. Cell Prolif. 2018, 51, e12427. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Boronat, A.; Rodríguez-Concepción, M. Terpenoid biosynthesis in prokaryotes. Adv. Biochem. Eng. Biotechnol. 2015, 148, 3–18. [Google Scholar]
- Liu, Z.; Cecarini, V.; Cuccioloni, M.; Bonfili, L.; Gong, C.; Angeletti, M.; Eleuteri, A.M. Ginsenosides Rg1 and Rg2 Activate Autophagy and Attenuate Oxidative Stress in Neuroblastoma Cells Overexpressing Aβ(1-42). Antioxidants 2024, 13, 310. [Google Scholar] [CrossRef] [Scilit]
- Gallily, R.; Yekhtin, Z.; Hanuš, L.O. The Anti-Inflammatory Properties of Terpenoids from Cannabis. Cannabis Cannabinoid Res. 2018, 3, 282–290. [Google Scholar] [CrossRef] [Scilit]
- Taban Akça, K.; Çınar Ayan, İ.; Çetinkaya, S.; Miser Salihoğlu, E.; Süntar, İ. Autophagic mechanisms in longevity intervention: Role of natural active compounds. Expert. Rev. Mol. Med. 2023, 25, e13. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gutiérrez-del-Río, I.; López-Ibáñez, S.; Magadán-Corpas, P.; Fernández-Calleja, L.; Pérez-Valero, Á.; Tuñón-Granda, M.; Miguélez, E.M.; Villar, C.J.; Lombó, F. Terpenoids and polyphenols as natural antioxidant agents in food preservation. Antioxidants 2021, 10, 1264. [Google Scholar] [CrossRef] [Scilit]
- Groeger, A.L.; Freeman, B.A. Signaling actions of electrophiles: Anti-inflammatory therapeutic candidates. Mol. Interv. 2010, 10, 39. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ling, T.; Boyd, L.; Rivas, F. Triterpenoids as reactive oxygen species modulators of cell fate. Chem. Res. Toxicol. 2022, 35, 569–584. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, J.; Yang, J.; Cao, M.; Zhao, Z.; Cao, B.; Yu, S. The potential roles of Nrf2/Keap1 signaling in anticancer drug interactions. Curr. Res. Pharmacol. Drug Discov. 2021, 2, 100028. [Google Scholar] [CrossRef] [Scilit]
- Szymczak, K.; Zakłos-Szyda, M.; Mietlińska, K.; Eliašová, A.; Jodłowska, I.; Gruľová, D.; Hodun, G.; Bonikowski, R. Old Apple Cultivars as a Natural Source of Phenolics and Triterpenoids with Cytoprotective Activity on Caco-2 and HepG2 Cells. Foods 2024, 13, 1014. [Google Scholar] [CrossRef] [Scilit]
- Singh, B.K.; Tripathi, M.; Chaudhari, B.P.; Pandey, P.K.; Kakkar, P. Natural terpenes prevent mitochondrial dysfunction, oxidative stress and release of apoptotic proteins during nimesulide-hepatotoxicity in rats. PLoS ONE 2012, 7, e34200. [Google Scholar] [CrossRef] [Scilit]
- Adom, K.K.; Liu, R.H. Rapid peroxyl radical scavenging capacity (PSC) assay for assessing both hydrophilic and lipophilic antioxidants. J. Agric. Food Chem. 2005, 53, 6572–6580. [Google Scholar] [CrossRef] [Scilit]
- Lee, W.-L.; Huang, J.-Y.; Shyur, L.-F. Phytoagents for cancer management: Regulation of nucleic acid oxidation, ROS, and related mechanisms. Oxidative Med. Cell. Longev. 2013, 2013, 925804. [Google Scholar] [CrossRef] [Scilit]
- Bansal, M.; Bhadouria, U.; Garg, S.; Sood, T.; Sharma, T. Carnosic acid: Perspectives on contemporary applications, molecular mechanisms, and therapeutic potential. Rev. Bras. De Farmacogn. 2025, 35, 333–344. [Google Scholar] [CrossRef] [Scilit]
- Shen, S.; Zhang, Y.; Zhang, R.; Tu, X.; Gong, X. Ursolic acid induces autophagy in U87MG cells via ROS-dependent endoplasmic reticulum stress. Chem. Biol. Interact. 2014, 218, 28–41. [Google Scholar] [CrossRef] [Scilit]
- Hu, C.; Cao, Y.; Li, P.; Tang, X.; Yang, M.; Gu, S.; Xiong, K.; Li, T.; Xiao, T. Oleanolic Acid Induces Autophagy and Apoptosis via the AMPK-mTOR Signaling Pathway in Colon Cancer. J. Oncol. 2021, 2021, 8281718. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wu, C.-F.; Ouyang, L.-X.; Zhang, W.-H.; Yang, S.; Zhong, X.-X.; Lin, Y.; Fan, S.; Li, P.; Liang, Z.-J. Andrographolide suppresses chondrosarcoma cell migration and invasion by inhibiting the PI3K/Akt/mTOR signaling pathway and activating autophagy. Front. Oncol. 2025, 15, 1622666. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, J.; Su, H.; Qu, Q.-M. Carnosic acid prevents beta-amyloid-induced injury in human neuroblastoma sh-sy5y cells via the induction of autophagy. Neurochem. Res. 2016, 41, 2311–2323. [Google Scholar] [CrossRef] [Scilit]
- Yang, C.; Su, C.; Iyaswamy, A.; Krishnamoorthi, S.K.; Zhu, Z.; Yang, S.; Tong, B.C.; Liu, J.; Sreenivasmurthy, S.G.; Guan, X. Celastrol enhances transcription factor EB (TFEB)-mediated autophagy and mitigates Tau pathology: Implications for Alzheimer’s disease therapy. Acta Pharm. Sin. B 2022, 12, 1707–1722. [Google Scholar] [CrossRef] [Scilit]
- Wan, X.; Li, C.; Tan, Y.H.; Zuo, S.Q.; Deng, F.M.; Sun, J.; Liu, Y.L. Dihydroartemisinin eliminates senescent cells by promoting autophagy-dependent ferroptosis via AMPK/mTOR signaling pathway. Cell Biol. Int. 2024, 48, 726–736. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, J.; Jiang, M.; Yu, Z.; Xiong, C.; Pan, J.; Cai, Z.; Xu, N.; Zhou, X.; Huang, Y.; Yang, Z. Artemisinin relieves osteoarthritis by activating mitochondrial autophagy through reducing TNFSF11 expression and inhibiting PI3K/AKT/mTOR signaling in cartilage. Cell. Mol. Biol. Lett. 2022, 27, 62. [Google Scholar] [CrossRef] [Scilit]
- Zhao, F.; Huang, W.; Zhang, Z.; Mao, L.; Han, Y.; Yan, J.; Lei, M. Triptolide induces protective autophagy through activation of the CaMKKβ-AMPK signaling pathway in prostate cancer cells. Oncotarget 2016, 7, 5366–5382. [Google Scholar] [CrossRef] [Scilit]
- Liu, X.; Chen, J.; Sun, N.; Li, N.; Zhang, Z.; Zheng, T.; Li, Z. Ginsenoside Rb1 ameliorates autophagy via the AMPK/mTOR pathway in renal tubular epithelial cells in vitro and in vivo. Int. J. Biol. Macromol. 2020, 163, 996–1009. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jiang, Q.; Lu, M.; Li, J.; Zhu, Z. Ginkgolide B Protects Cardiomyocytes from Angiotensin II-Induced Hypertrophy via Regulation of Autophagy through SIRT1-FoxO1. Cardiovasc. Ther. 2021, 2021, 5554569. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Galasso, C.; Corinaldesi, C.; Sansone, C. Carotenoids from Marine Organisms: Biological Functions and Industrial Applications. Antioxidants 2017, 6, 96. [Google Scholar] [CrossRef] [Scilit]
- Ferreira, Y.A.M.; Jamar, G.; Estadella, D.; Pisani, L.P. Role of carotenoids in adipose tissue through the AMPK-mediated pathway. Food Funct. 2023, 14, 3454–3462. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dewanjee, S.; Bhattacharjee, N.; Chakraborty, P.; Bhattacharjee, S. Carotenoids as antioxidants. In Carotenoids: Structure and Function in the Human Body; Springer: Berlin/Heidelberg, Germany, 2021; pp. 447–473. [Google Scholar]
- Rodriguez-Amaya, D.B. Food Carotenoids: Chemistry, Biology and Technology; John Wiley & Sons: Hoboken, NJ, USA, 2015. [Google Scholar]
- Polyakov, N.E.; Focsan, A.L.; Gao, Y.; Kispert, L.D. The endless world of carotenoids—Structural, chemical and biological aspects of some rare carotenoids. Int. J. Mol. Sci. 2023, 24, 9885. [Google Scholar] [CrossRef] [Scilit]
- Fong, C.W. The Origin of The Antioxidant Capacity Against Oxidative and Photooxidative Stress, Singlet Oxygen Reactivity, and the Excited States in Skin and Eye Related Diseases of Astaxanthin and Other Carotenoids, Isomers and Esters in The Cell Membrane and Cytosol; Eigenenergy Adelaide South Australia: Adelaide, Australia, 2023. [Google Scholar]
- Black, H.S.; Boehm, F.; Edge, R.; Truscott, T.G. The benefits and risks of certain dietary carotenoids that exhibit both anti-and pro-oxidative mechanisms—A comprehensive review. Antioxidants 2020, 9, 264. [Google Scholar] [CrossRef] [Scilit]
- Boehm, F.; Edge, R.; Truscott, T.G. Photochemical and photophysical properties of carotenoids and reactive oxygen species: Contradictions relating to skin and vision. Oxygen 2023, 3, 322–335. [Google Scholar] [CrossRef] [Scilit]
- Böhm, F.; Edge, R.; Truscott, G. Interactions of dietary carotenoids with activated (singlet) oxygen and free radicals: Potential effects for human health. Mol. Nutr. Food Res. 2012, 56, 205–216. [Google Scholar] [CrossRef] [Scilit]
- Granado-Lorencio, F.; Blanco-Navarro, I.; Pérez-Sacristán, B.; Hernández-Álvarez, E. Biomarkers of carotenoid bioavailability. Food Res. Int. 2017, 99, 902–916. [Google Scholar] [CrossRef] [Scilit]
- Tsuchiya, M.; Scita, G.; Freisleben, H.J.; Kagan, V.E.; Packer, L. Antioxidant radical-scavenging activity of carotenoids and retinoids compared to alpha-tocopherol. Methods Enzym. 1992, 213, 460–472. [Google Scholar]
- de Souza Guedes, L.; Martinez, R.M.; Bou-Chacra, N.A.; Velasco, M.V.R.; Rosado, C.; Baby, A.R. An Overview on Topical Administration of Carotenoids and Coenzyme Q10 Loaded in Lipid Nanoparticles. Antioxidants 2021, 10, 1034. [Google Scholar] [CrossRef] [Scilit]
- Bakac, E.R.; Percin, E.; Gunes-Bayir, A.; Dadak, A. A Narrative Review: The Effect and Importance of Carotenoids on Aging and Aging-Related Diseases. Int. J. Mol. Sci. 2023, 24, 15199. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- El-Marasy, S.A.; Farouk, H.; Khattab, M.S.; Moustafa, P.E. Beta-carotene ameliorates diabetic nephropathy in rats: Involvement of AMPK/SIRT1/autophagy pathway. Immunopharmacol. Immunotoxicol. 2024, 46, 763–772. [Google Scholar] [CrossRef] [Scilit]
- Tan, C.; Chen, J.; Tu, T.; Chen, L.; Zou, J. Lycopene inhibits pyroptosis of endothelial progenitor cells induced by ox-LDL through the AMPK/mTOR/NLRP3 pathway. Open Med. 2024, 19, 20240973. [Google Scholar] [CrossRef] [Scilit]
- Fung, F.K.; Law, B.Y.; Lo, A.C. Lutein Attenuates Both Apoptosis and Autophagy upon Cobalt (II) Chloride-Induced Hypoxia in Rat Műller Cells. PLoS ONE 2016, 11, e0167828. [Google Scholar] [CrossRef] [Scilit]
- Zou, X.; Gao, J.; Zheng, Y.; Wang, X.; Chen, C.; Cao, K.; Xu, J.; Li, Y.; Lu, W.; Liu, J.; et al. Zeaxanthin induces Nrf2-mediated phase II enzymes in protection of cell death. Cell Death Dis. 2014, 5, e1218. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gao, H.; Lv, Y.; Liu, Y.; Li, J.; Wang, X.; Zhou, Z.; Tipoe, G.L.; Ouyang, S.; Guo, Y.; Zhang, J.; et al. Wolfberry-Derived Zeaxanthin Dipalmitate Attenuates Ethanol-Induced Hepatic Damage. Mol. Nutr. Food Res. 2019, 63, e1801339. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Babalola, J.A.; Lang, M.; George, M.; Stracke, A.; Tam-Amersdorfer, C.; Itxaso, I.; Lucija, D.; Tadic, J.; Schilcher, I.; Loeffler, T.; et al. Astaxanthin enhances autophagy, amyloid beta clearance and exerts anti-inflammatory effects in in vitro models of Alzheimer’s disease-related blood brain barrier dysfunction and inflammation. Brain Res. 2023, 1819, 148518. [Google Scholar] [CrossRef] [Scilit]
- Jang, E.J.; Kim, S.C.; Lee, J.H.; Lee, J.R.; Kim, I.K.; Baek, S.Y.; Kim, Y.W. Fucoxanthin, the constituent of Laminaria japonica, triggers AMPK-mediated cytoprotection and autophagy in hepatocytes under oxidative stress. BMC Complement. Altern. Med. 2018, 18, 97. [Google Scholar] [CrossRef] [Scilit]
- Noguchi, M.; Kitakaze, T.; Kobayashi, Y.; Mukai, K.; Harada, N.; Yamaji, R. β-Cryptoxanthin Improves p62 Accumulation and Muscle Atrophy in the Soleus Muscle of Senescence-Accelerated Mouse-Prone 1 Mice. Nutrients 2020, 12, 2180. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, Z.; Liu, W.; Zhang, M.; Yan, J.; Fei, J.; Zhang, K.; Dong, S. Canthaxanthin Mitigates Cardiovascular Senescence in Vitro and in Vivo. Front. Biosci. 2024, 29, 70. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wani, A.; Al Rihani, S.B.; Sharma, A.; Weadick, B.; Govindarajan, R.; Khan, S.U.; Sharma, P.R.; Dogra, A.; Nandi, U.; Reddy, C.N.; et al. Crocetin promotes clearance of amyloid-β by inducing autophagy via the STK11/LKB1-mediated AMPK pathway. Autophagy 2021, 17, 3813–3832. [Google Scholar] [CrossRef] [Scilit]
- Li, J.; Yang, Y.; Wei, S.; Chen, L.; Xue, L.; Tian, H.; Tao, S. Bixin Protects Against Kidney Interstitial Fibrosis Through Promoting STAT6 Degradation. Front. Cell Dev. Biol. 2020, 8, 576988. [Google Scholar] [CrossRef] [Scilit]
- Noce, A.; Di Lauro, M.; Di Daniele, F.; Pietroboni Zaitseva, A.; Marrone, G.; Borboni, P.; Di Daniele, N. Natural Bioactive Compounds Useful in Clinical Management of Metabolic Syndrome. Nutrients 2021, 13, 630. [Google Scholar] [CrossRef] [Scilit]
- Liu, Z.; Hu, M. Natural polyphenol disposition via coupled metabolic pathways. Expert. Opin. Drug Metab. Toxicol. 2007, 3, 389–406. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yang, J.; Li, K.; He, D.; Gu, J.; Xu, J.; Xie, J.; Zhang, M.; Liu, Y.; Tan, Q.; Zhang, J. Toward a better understanding of metabolic and pharmacokinetic characteristics of low-solubility, low-permeability natural medicines. Drug Metab. Rev. 2020, 52, 19–43. [Google Scholar] [CrossRef] [Scilit]
- Ademowo, O.S.; Oyebode, O.; Edward, R.; Conway, M.E.; Griffiths, H.R.; Dias, I.H.K. Effects of carotenoids on mitochondrial dysfunction. Biochem. Soc. Trans. 2024, 52, 65–74. [Google Scholar] [CrossRef] [Scilit]
- Feng, X.; Wang, K.; Cao, S.; Ding, L.; Qiu, F. Pharmacokinetics and Excretion of Berberine and Its Nine Metabolites in Rats. Front. Pharmacol. 2020, 11, 594852. [Google Scholar] [CrossRef] [Scilit]
- Zou, D.; Zhao, Z.; Li, L.; Min, Y.; Zhang, D.; Ji, A.; Jiang, C.; Wei, X.; Wu, X. A comprehensive review of spermidine: Safety, health effects, absorption and metabolism, food materials evaluation, physical and chemical processing, and bioprocessing. Compr. Rev. Food Sci. Food Saf. 2022, 21, 2820–2842. [Google Scholar] [CrossRef] [Scilit]
- Zhang, H.; Yan, Q.; Wang, X.; Chen, X.; Chen, Y.; Du, J.; Chen, L. The Role of Mitochondria in Liver Ischemia-Reperfusion Injury: From Aspects of Mitochondrial Oxidative Stress, Mitochondrial Fission, Mitochondrial Membrane Permeable Transport Pore Formation, Mitophagy, and Mitochondria-Related Protective Measures. Oxidative Med. Cell. Longev. 2021, 2021, 6670579. [Google Scholar] [CrossRef] [Scilit]
- Oteiza, P.I.; Erlejman, A.G.; Verstraeten, S.V.; Keen, C.L.; Fraga, C.G. Flavonoid-membrane interactions: A protective role of flavonoids at the membrane surface? J. Immunol. Res. 2005, 12, 19–25. [Google Scholar] [CrossRef] [Scilit]
- Cheng, H.; Zhang, D.; Wu, J.; Liu, J.; Zhou, Y.; Tan, Y.; Feng, W.; Peng, C. Interactions between gut microbiota and polyphenols: A mechanistic and metabolomic review. Phytomedicine 2023, 119, 154979. [Google Scholar] [CrossRef] [Scilit]
- García-Aguilar, A.; Palomino, O.; Benito, M.; Guillén, C. Dietary Polyphenols in Metabolic and Neurodegenerative Diseases: Molecular Targets in Autophagy and Biological Effects. Antioxidants 2021, 10, 142. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Siraj, M.A.; Islam, M.A.; Al Fahad, M.A.; Kheya, H.R.; Xiao, J.; Simal-Gandara, J. Cancer chemopreventive role of dietary terpenoids by modulating Keap1-Nrf2-ARE signaling system—A comprehensive update. Appl. Sci. 2021, 11, 10806. [Google Scholar] [CrossRef] [Scilit]
- Hu, Y.; Chen, X.; Zhao, Q.; Li, G.; Zhang, H.; Ma, Z.; Yu, H.; Zeng, Q.; Zhang, H.; Xu, D. Berberine improves cardiac insufficiency through AMPK/PGC-1α signaling-mediated mitochondrial homeostasis and apoptosis in HFpEF mice. Int. Immunopharmacol. 2025, 155, 114613. [Google Scholar] [CrossRef] [Scilit]
- Arcaro, A.; Lepore, A.; Cetrangolo, G.P.; Paventi, G.; Ames, P.R.J.; Gentile, F. A reassessment of sarcopenia from a redox perspective as a basis for preventive and therapeutic interventions. Int. J. Mol. Sci. 2025, 26, 7787. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Salehi, B.; Azzini, E.; Zucca, P.; Maria Varoni, E.V.; Anil Kumar, N.; Dini, L.; Panzarini, E.; Rajkovic, J.; Valere Tsouh Fokou, P.; Peluso, I. Plant-derived bioactives and oxidative stress-related disorders: A key trend towards healthy aging and longevity promotion. Appl. Sci. 2020, 10, 947. [Google Scholar] [CrossRef] [Scilit]
- Qi, T.; Zhang, K.; Zhang, J.; Ma, Y.; Hou, N.; Sun, X.; Han, F.; Sheng, S.; Kan, C. Aging-related obesity: Unveiling mitochondrial and metabolic dysfunction. Curr. Nutr. Rep. 2025, 14, 94. [Google Scholar] [CrossRef] [Scilit]
- Brimson, J.M.; Prasanth, M.I.; Malar, D.S.; Thitilertdecha, P.; Kabra, A.; Tencomnao, T.; Prasansuklab, A. Plant polyphenols for aging health: Implication from their autophagy modulating properties in age-associated diseases. Pharmaceuticals 2021, 14, 982. [Google Scholar] [CrossRef] [Scilit]
- Khater, S.; Almanaa, T.; Fattah, D.; Khamis, T.; Seif, M.; Dahran, N.; Alqahtani, L.; Metwally, M.; Mostafa, M.; Albedair, R. Liposome-encapsulated berberine alleviates liver injury in type 2 diabetes via promoting AMPK/mTOR-mediated autophagy and reducing ER stress: Morphometric and immunohistochemical scoring. Antioxidants 2023, 12, 1220. [Google Scholar] [CrossRef] [Scilit]
- Akter, S. Examining the Role of Carotenoids and Retinoids in Modulating Cellular Response to Oxidative Stress: An Evidence-based Approach. Ph.D. Thesis, Laurentian University Library & Archives, Greater Sudbury, ON, Canada, 2025. [Google Scholar]
- Das, D.M.K.; Mitra, A.; Zaky, M.Y.; Pathak, S.; Banerjee, A. A review on the efficacy of plant-derived bio-active compounds curcumin and aged garlic extract in modulating cancer and age-related diseases. Curr. Rev. Clin. Exp. Pharmacol. Former. Curr. Clin. Pharmacol. 2024, 19, 146–162. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, Z.; Quan, W.; Zeng, M.; Wang, Z.; Chen, Q.; Chen, J.; Christian, M.; He, Z. Regulation of autophagy by plant-based polyphenols: A critical review of current advances in glucolipid metabolic diseases and food industry applications. Food Front. 2023, 4, 1039–1067. [Google Scholar] [CrossRef] [Scilit]
- Park, S.-H.; Lee, D.-H.; Lee, D.-H.; Jung, C.H. Scientific evidence of foods that improve the lifespan and healthspan of different organisms. Nutr. Res. Rev. 2024, 37, 169–178. [Google Scholar] [CrossRef] [Scilit]
- Xu, T.-T.; Li, H.; Dai, Z.; Lau, G.K.; Li, B.-Y.; Zhu, W.-L.; Liu, X.-Q.; Liu, H.-F.; Cai, W.-W.; Huang, S.-Q. Spermidine and spermine delay brain aging by inducing autophagy in SAMP8 mice. Aging 2020, 12, 6401. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bensalem, J.; Hattersley, K.J.; Hein, L.K.; Teong, X.T.; Carosi, J.M.; Hassiotis, S.; Grose, R.H.; Fourrier, C.; Heilbronn, L.K.; Sargeant, T.J. Measurement of autophagic flux in humans: An optimized method for blood samples. Autophagy 2021, 17, 3238–3255. [Google Scholar] [CrossRef] [Scilit]
- Andreux, P.A.; Blanco-Bose, W.; Ryu, D.; Burdet, F.; Ibberson, M.; Aebischer, P.; Auwerx, J.; Singh, A.; Rinsch, C. The mitophagy activator urolithin A is safe and induces a molecular signature of improved mitochondrial and cellular health in humans. Nat. Metab. 2019, 1, 595–603. [Google Scholar] [CrossRef] [Scilit]
- Schwarz, C.; Benson, G.S.; Horn, N.; Wurdack, K.; Grittner, U.; Schilling, R.; Märschenz, S.; Köbe, T.; Hofer, S.J.; Magnes, C.; et al. Effects of Spermidine Supplementation on Cognition and Biomarkers in Older Adults With Subjective Cognitive Decline: A Randomized Clinical Trial. JAMA Netw. Open 2022, 5, e2213875. [Google Scholar] [CrossRef] [Scilit]
- Alsaleh, G.; Panse, I.; Swadling, L.; Zhang, H.; Richter, F.C.; Meyer, A.; Lord, J.; Barnes, E.; Klenerman, P.; Green, C.; et al. Autophagy in T cells from aged donors is maintained by spermidine and correlates with function and vaccine responses. eLife 2020, 9, e57950. [Google Scholar] [CrossRef] [Scilit]
- Park, D.; Jeong, H.; Lee, M.N.; Koh, A.; Kwon, O.; Yang, Y.R.; Noh, J.; Suh, P.G.; Park, H.; Ryu, S.H. Resveratrol induces autophagy by directly inhibiting mTOR through ATP competition. Sci. Rep. 2016, 6, 21772. [Google Scholar] [CrossRef] [Scilit]
- Han, J.; Pan, X.Y.; Xu, Y.; Xiao, Y.; An, Y.; Tie, L.; Pan, Y.; Li, X.J. Curcumin induces autophagy to protect vascular endothelial cell survival from oxidative stress damage. Autophagy 2012, 8, 812–825. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhou, J.; Farah, B.L.; Sinha, R.A.; Wu, Y.; Singh, B.K.; Bay, B.H.; Yang, C.S.; Yen, P.M. Epigallocatechin-3-gallate (EGCG), a green tea polyphenol, stimulates hepatic autophagy and lipid clearance. PLoS ONE 2014, 9, e87161. [Google Scholar] [CrossRef] [Scilit]
- Tabanelli, R.; Brogi, S.; Calderone, V. Improving curcumin bioavailability: Current strategies and future perspectives. Pharmaceutics 2021, 13, 1715. [Google Scholar] [CrossRef] [Scilit]
- Tabibzadeh, S. Role of autophagy in aging: The good, the bad, and the ugly. Aging Cell 2023, 22, e13753. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Shu, F.; Xiao, H.; Li, Q.-N.; Ren, X.-S.; Liu, Z.-G.; Hu, B.-W.; Wang, H.-S.; Wang, H.; Jiang, G.-M. Epigenetic and post-translational modifications in autophagy: Biological functions and therapeutic targets. Signal Transduct. Target. Ther. 2023, 8, 32. [Google Scholar] [CrossRef] [Scilit] [PubMed]
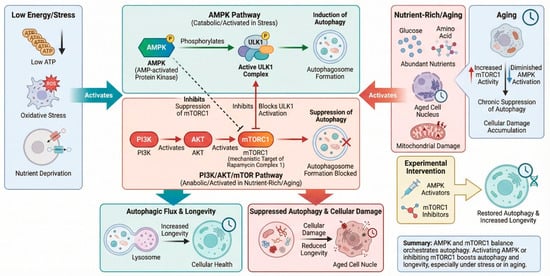
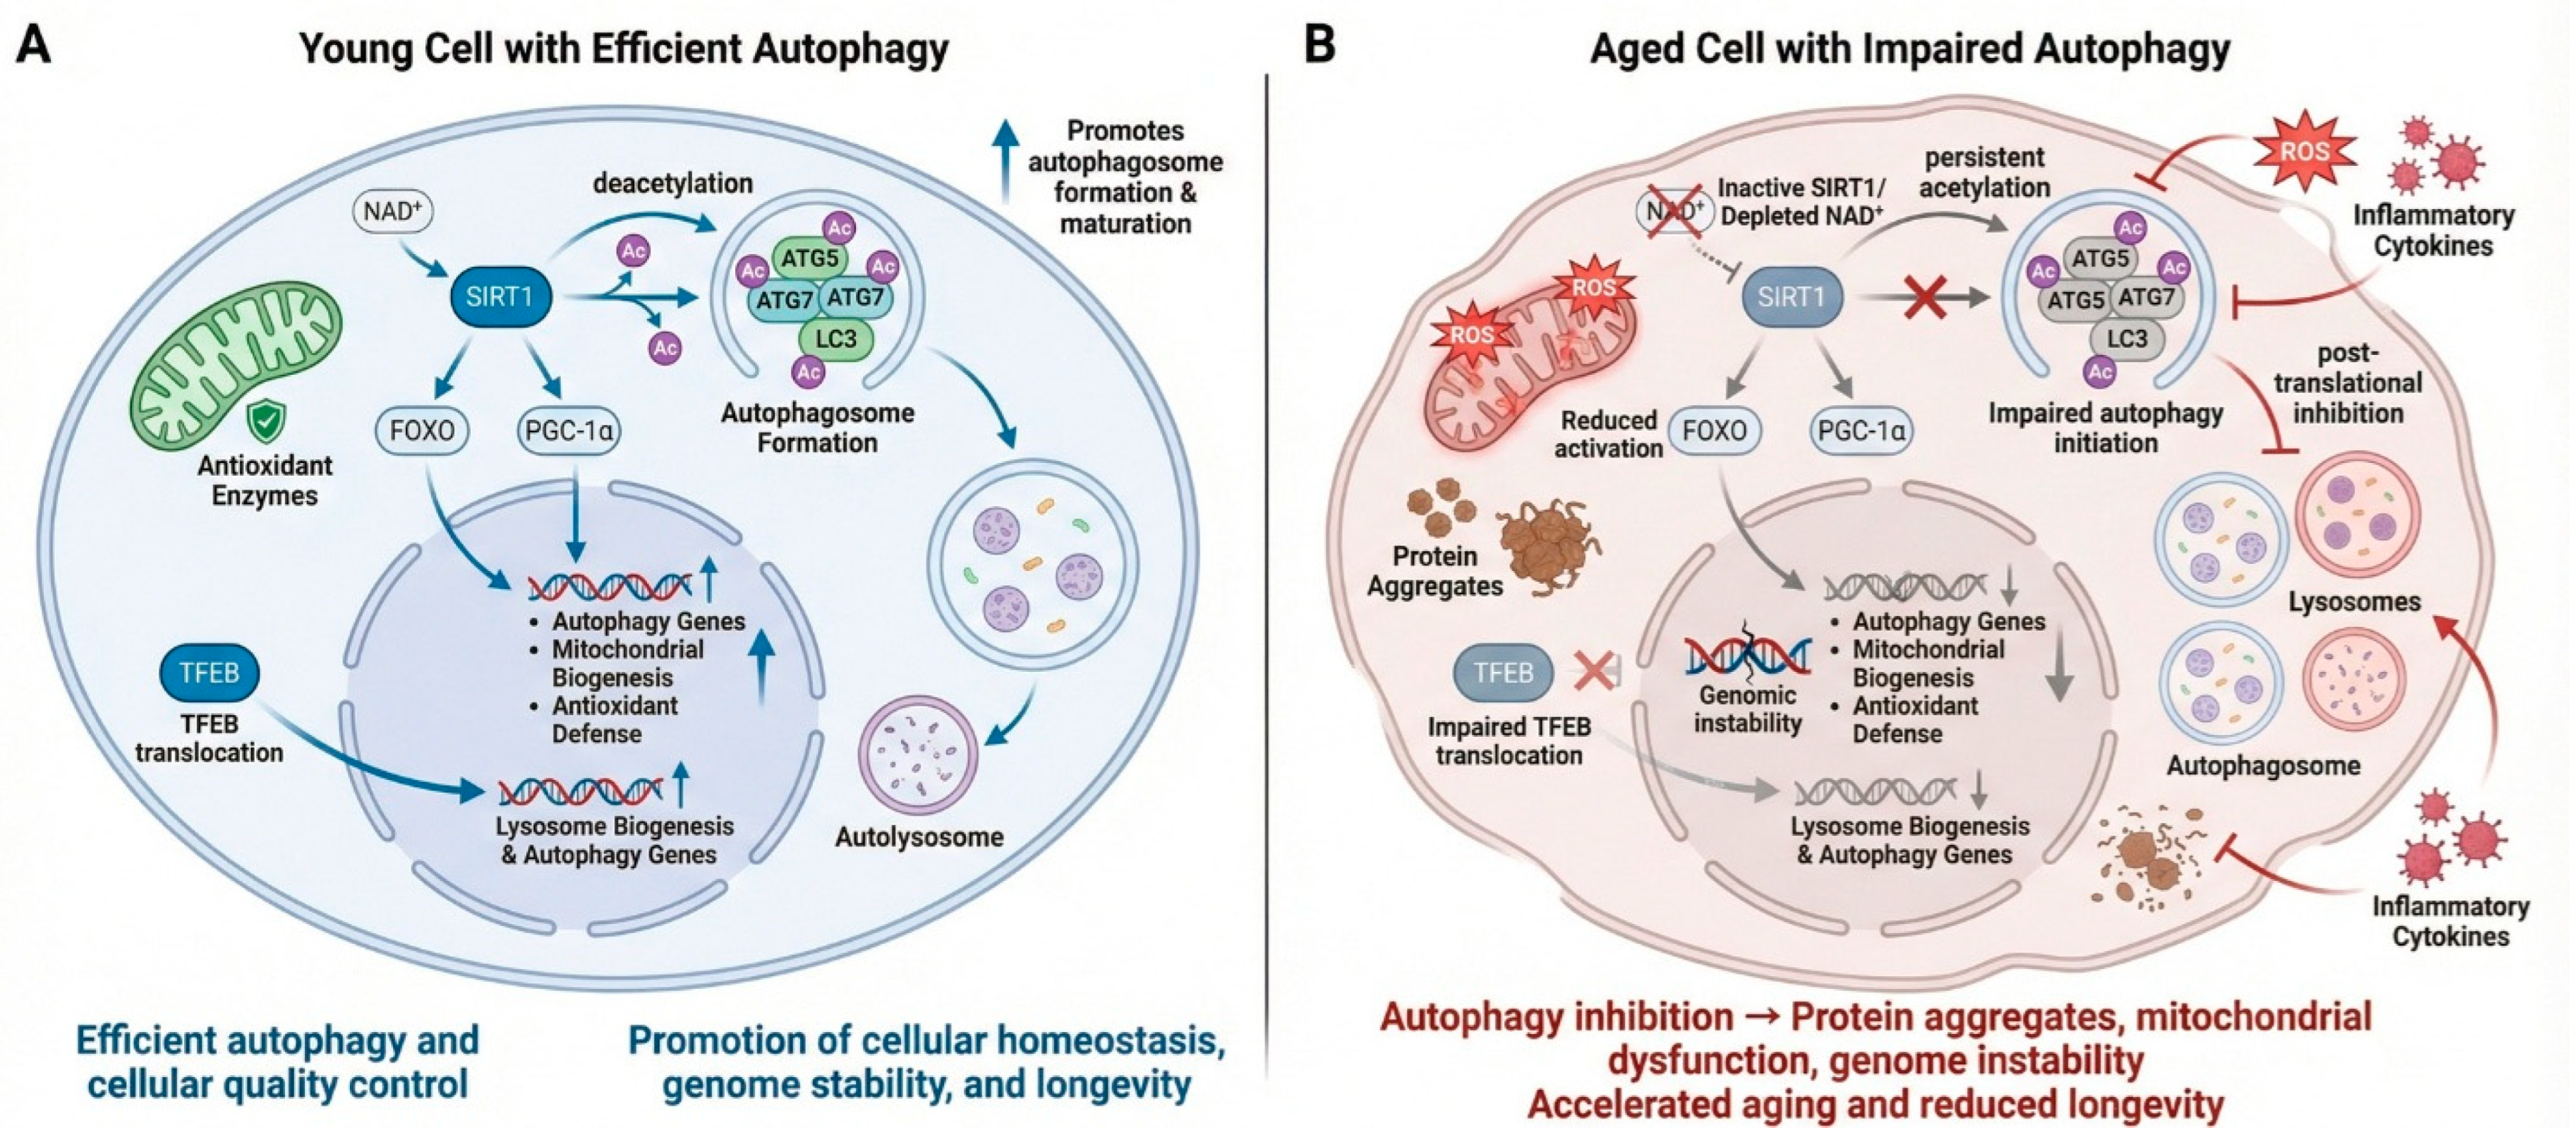
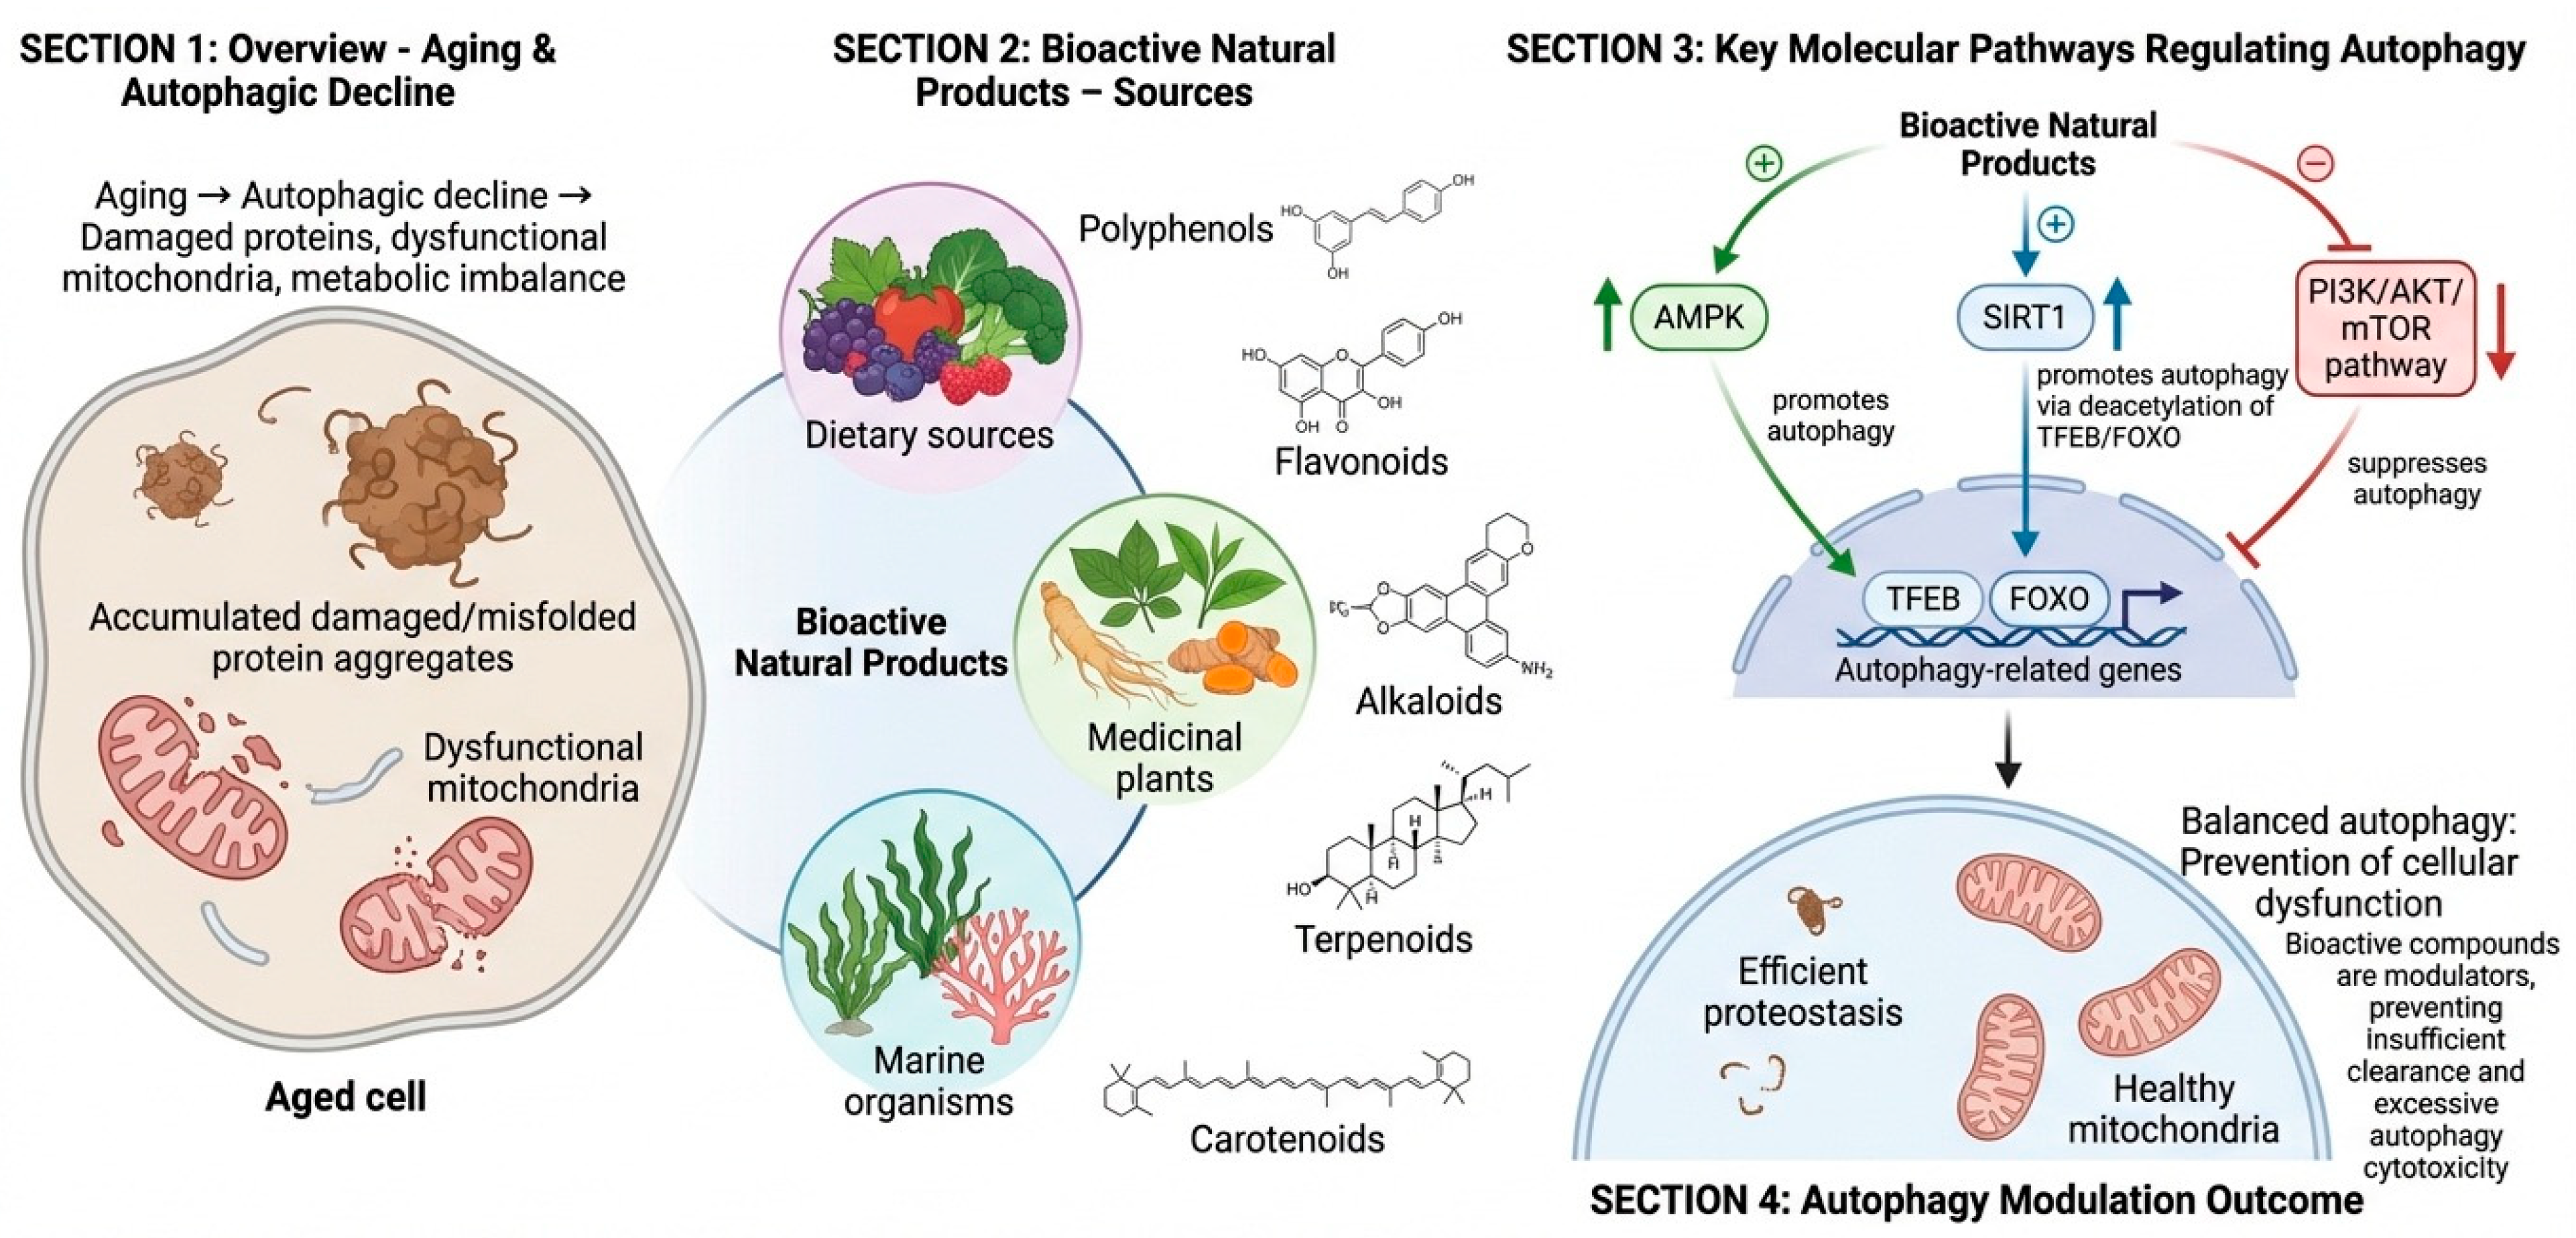
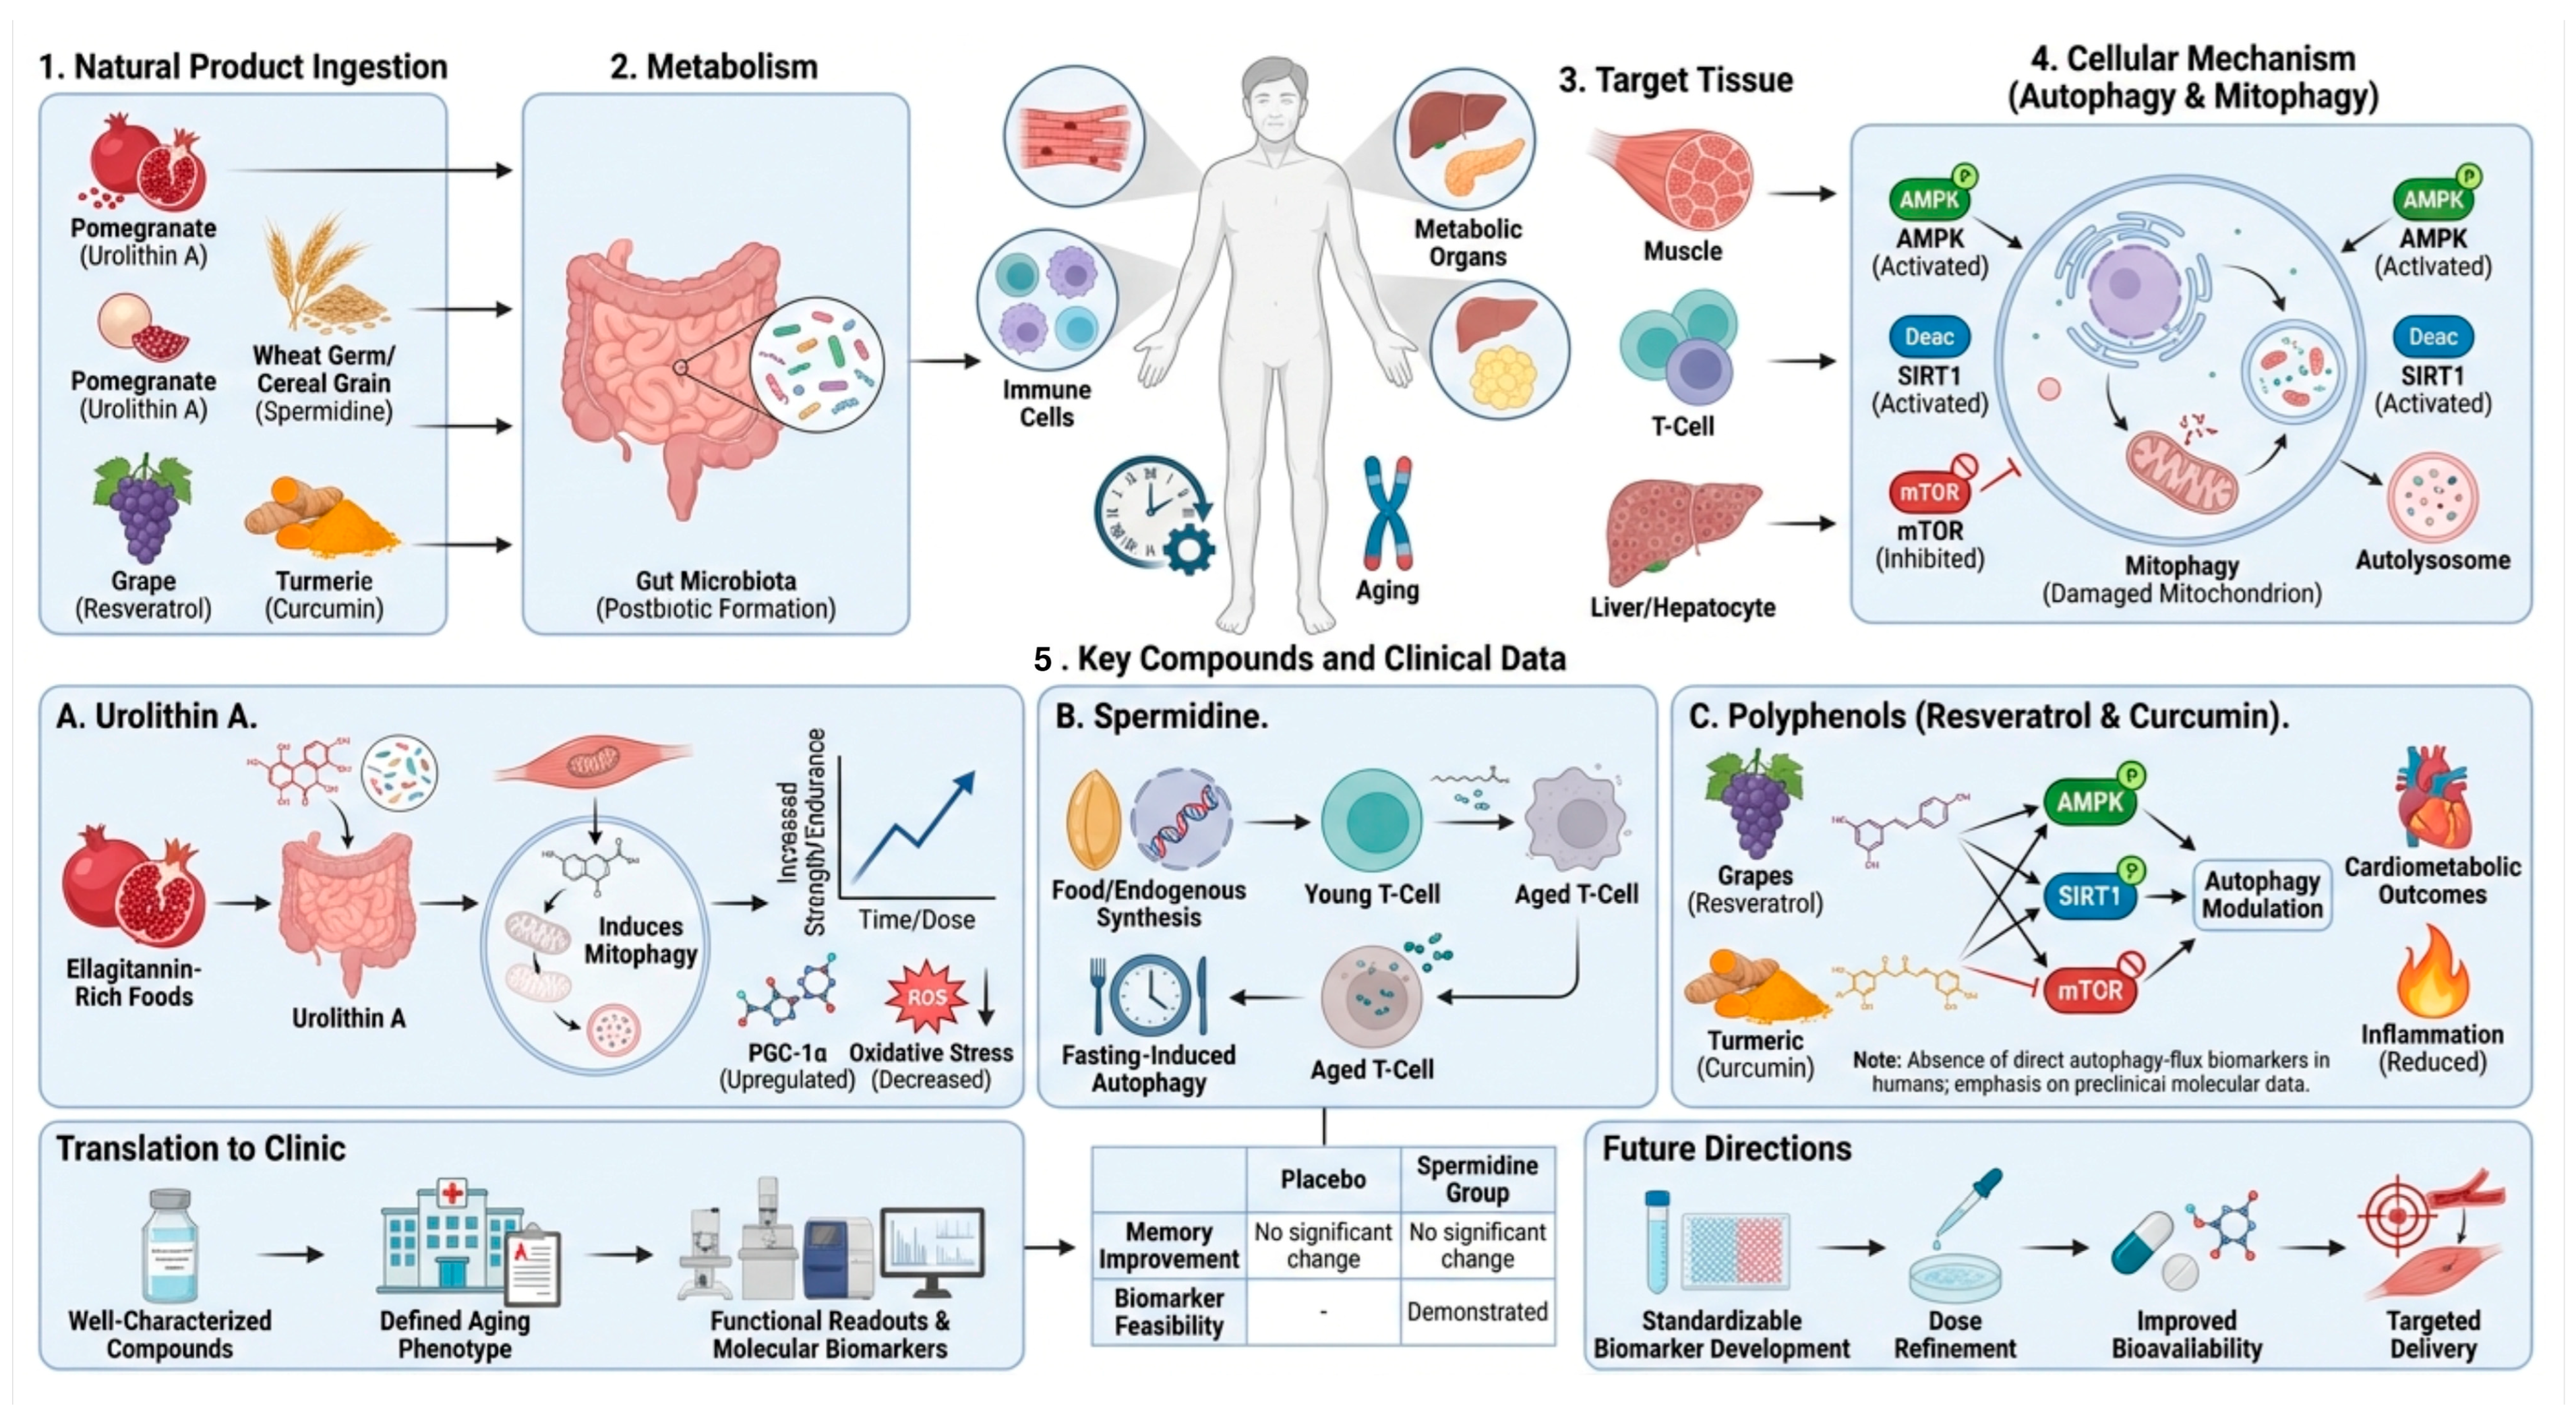
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.