


Abstract
In northeast British Columbia (BC), Canada, industrial forestry is gradually converting 10+ M ha of broadleaf–conifer (mixedwood) boreal forest to conifer plantations. This is due in part to governmental free-to-grow (FTG) regulations, which specify a minimum competition-free radius around conifer crop trees. FTG implementation is a poor investment; it reduces stand biodiversity and productivity and infringes on Indigenous Treaty Rights. Trials were established on three geographically separated boreal sites with no stand management (brushing) since planting. The goal was to determine the effect of FTG criteria on conifer growth in mixedwoods compared to growth of pure conifer stands using the BC Government growth model TIPSY (Table Interpolation Program of Stand Yield) projections. At trial establishment, less than a third of trees were FTG. The number of FTG trees increased at the last measurement but only reached 50 percent on one site. After a decade, conifer DBH (diameter at breast height) growth and stand productivity met or exceeded the model projection regardless of the initial FTG status. The DBH relative growth rate (RGR) indicated that spruce DBH growth was not impacted by competitors. These observations suggest that brushing on similar sites to meet timber objectives is likely unnecessary. Maintaining mixedwood stands supports greater biodiversity and carbon storage, and this approach better aligns with an Indigenous world view and Treaty Rights. There is an opportunity in northeast BC to shift forest management from conifer-based performance metrics to prioritizing ecological resilience and long-term forest health and productivity.
1. Introduction
The 10+ M ha of forest on the Alberta Plateau in northern British Columbia (BC) are primarily mixedwoods of broadleaves and conifers but partly due to free-to-grow (FTG) criteria there has been a conversion to pure conifer stands [1,2,3]. The FTG status of plantations in northeast BC has been a point of contention for more than a decade because of the conversion to conifers [1,2]. In addition to the FTG criteria, economics and silviculture strategy generally dictates pure conifer management in reforested stands [4] but when commercially viable, there is a possibility for a broadleaf harvest [5].
The development of FTG standards, which are stocking standards and not regeneration standards reflects the conifer bias where a regenerating plantation’s performance is measured against a pure conifer stand’s growth [4,6,7]. To achieve FTG, at a minimum, there must be no competition within a 1 m cylinder around the measured tree and extending to more than two-thirds of its height [7]. The assumption underlying FTG is that there is a connection between sample metrics (density) and management goals (volume) [2] but to date the link has not been established [8,9,10]. As a result, FTG standards can result in forest managers applying broadcast vegetation removal (brushing) treatments to avoid administrative actions [4]. If a stand is not FTG, the licence holder is liable for its success until it is FTG. This leaves little incentive for retaining lower valued broadleaves. It ignores the successional path of this forest type [11], negatively impacts biodiversity [12,13], and it is inconsistent with traditional values and land use of First Nations [14]. The result is forest simplification [4]. It also may not conform to the United Nations Declaration on the Rights of Indigenous Peoples (UNDRIP), which has been endorsed by the provincial government of BC [15]. A recent court decision specified that the lack of broadleaf species in reforestation contributed to reduced moose numbers in the Treaty 8 area (northeast BC), which does not support Indigenous Treaty Rights (https://www.mandellpinder.com/yahey-v-british-columbia-2021-bcsc-1287-canlii-case-summary/, accessed on 13 April 2026).
The current management approach is based on older reports of broadleaves negatively impacting conifer growth [16,17,18,19,20,21]. This may result in brushing because of the FTG criteria and this can be costly [4]. In northeast BC, after brushing, the future stand value was only positive with a real interest rate of two percent or less [3]—a lower return on investment than the industry expects. Also, in Scandinavia, mixed-species stands were found to have a better land expectation value than stands managed for a single species [22].
Not managing for mixedwoods has costs too [12]. The productivity of mixedwoods is considered to be greater than that of either species grown in a pure stand [2,23,24,25,26,27,28,29] and stands may have greater carbon storage potential [30,31,32]. Regardless of whether carbon storage has economic value, management of mixedwoods to mitigate climate change is a valuable option [33] and it could be a future revenue stream [30]. Mixedwoods provide a spectrum of ecological goods and services [34]. They have a positive impact on biodiversity [22,35,36] and specific ecological values, such as moose [37] and bird [38,39] habitats, and resistance to abiotic (fires, wind, and floods) and biotic (forest health) perturbations [5,22,35]. Maintaining these values is a high priority for First Nations [14].
The future climate of northeast BC is projected to have a small increase in precipitation and be warmer with a longer growing season [40]. It has been suggested [36,41,42] that mixedwoods could successfully respond to new climate regimes better than pure conifer stands, possibly showing greater resilience than pure conifers. The observation that conifers could be impacted to a greater degree than broadleaf species in the region by a changing climate argues for mixedwood management. Conifer habitat in northeast BC is projected to shift northward while broadleaf distribution will likely be static [43]. The southern boundary of the boreal forest (e.g., northeast BC) is projected to undergo greater climate stresses than other regions too [44].
This study aims to enhance our understanding of interactions between conifer crop trees (white spruce and Picea glauca (Moench) Voss) and associated broadleaf tree competition (trembling aspen, Populus tremuloides Michx., paper birch, and Betula papyifera Marsh) in northeast BC. A short-term objective is to determine if FTG metrics are adequate or need modification to be pertinent for forest management in northeast BC. A project goal is to limit ecological and economic costs, minimize the impact on First Nations’ traditional land use and Treaty Rights, while maintaining forest productivity.
2. Methods
2.1. The Site
The three sites are located east of the Rocky Mountains on the Alberta Plateau in BC, Canada (Table 1). They are even-aged broadleaf–conifer stands (mixedwoods) in the Boreal White and Black Spruce (BWBS) biogeoclimatic zone (BEC) [45]. Lacustrine clays dominate the soils of the sites. The Prophet River site is in the BWBS moist cool (mk) subzone and the other sites are in the moist warm (mw) subzone. The sites are mesic with gentle topography and uniform conifer distribution due to planting. As noted, a changing climate is projected to have the greatest effect on this part of the boreal forest [44]. For the region, the projection [40] suggests greater precipitation (MAP, 11%–19%), mean annual temperature (MAT, 1.9–4.7 °C), and frost-free (FF) period (25–40 days). Currently, precipitation is half snow and totals about 450 mm across the region; MAT from north to south ranges from 0 °C to +3 °C with extremes from −52 °C to +36 °C; and independent of latitude, FF ranges from 90 to 125 days.
Table 1.
Location of sites on the Alberta Plateau of northeast BC (longitude, latitude, year trial established (stand age since it was planted), and approximate site area).
The sites were reforested with containerized white spruce seedlings, a mid- to late-successional dominant [46] and intermediate shade-tolerant [47] species, and naturally regenerated broadleaves (trembling aspen or paper birch), which co-established with the planted conifer seedlings. At trial establishment, the sites’ post-planting age ranged from five to 18 years old (Table 1).
2.2. Plot Establishment and Measurement
Prior to plot establishment, no management activities other than planting had been implemented on the sites after logging. The nearest individual method was used to establish single tree sample plots [2,3,48]. The plots were established 25 m apart on a fixed bearing. The point was recorded using GPS and the nearest spruce tree became the plot centre and the crop tree (also recorded using GPS) was selected provided it was greater than 1.3 m in height (DBH point, diameter at breast height) and defect-free [2,3]. The latter was to ensure that crop tree growth reductions occurred due to competition (stand density) and not forest health. If there was a defect, the plot was moved a further 25 m on the bearing. Trials on similar sites indicated that until at least a 2 m radius was free of competition, there was no increase in crop tree DBH [2]. Our goal was to describe what occurred near the crop tree as 1 m is the FTG minimum competition-free radius. Rather than using 1 m radius plots, we enlarged it to a 1.785 m radius (10 m2) plot around each crop tree. This resulted in adequate stand stocking, 1000 SPH, and a competition area 3+ times greater than the FTG minimum. At trial initiation, all trees within the plot with a height greater than 1.3 m were measured for height and DBH and again during the winter of 2019–2020.
Site means were established for plot density (stems∙ha−1 or SPH), crop, and competitor tree DBH and height. Calculations determined basal area (BA), height-to-diameter ratio (HDR), and DBH relative growth rate (RGR). The DBH RGR is calculated per Equation (1) and reflects the plant’s growing environment [49]:
where DBH1 is the DBH at time 1 (T1) at the start of the trial and DBH2 is the DBH at time 2 (T2) during the winter of 2019–2020. DBH at trial establishment and its relation to the DBH RGR was tested with linear regression.
DBH RGR = (LN DBH2 − LN DBH1)/(T2 − T1)
2.3. Modeling
Nigh’s [50] growth intercept approach for young stands was used to estimate the stand site index at base age 50 (SIs). Trees with no competition within 2 m determined the SIs for the sites and were used to project the growth of a pure spruce stand at the site using TIPSY (Table Interpolation Program of Stand Yield) version 4.7 (downloaded on 4 January 2026, https://www2.gov.bc.ca/gov/content/industry/forestry/managing-our-forest-resources/forest-inventory/field-forms-and-software/software-download#tipsy) growth model developed by the BC Government. TIPSY retrieves and interpolates yield tables from its database, customizes the information, and displays summaries and graphics for a specific site, species, and management regime. Outputs include mean spruce height, volume, DBH, BA, and SPH. Attributes used in the TIPSY runs were SI, 1400 SPH of reforested white spruce as this was the planting norm when the sites were established, and model default forest health growth net downs (operational adjustment factors, OAF). OAF 1 is for nonproductive areas = 0.85 and OAF 2 is for decay, waste, and breakage = 0.95. The output is optimistic using these OAF values to gauge spruce growth in the mixed stands against the TIPSY projection for a pure spruce stand representative of each site’s productivity and age. TIPSY has been validated for white spruce in northeast BC and is used widely in timber supply determinations throughout the province. Based on FTG rationale, spruce DBH and basal area should be negatively impacted when grown with greater densities (SPH) of broadleaves.
Sites were analyzed separately.
3. Results
Because it is easy to measure and integrate tree physiological responses into environmental variation [51], DBH was used to detail crop tree response to broadleaf competition. Also when tree growth is compromised, diameter growth is the first energy sink to be shut down [52].
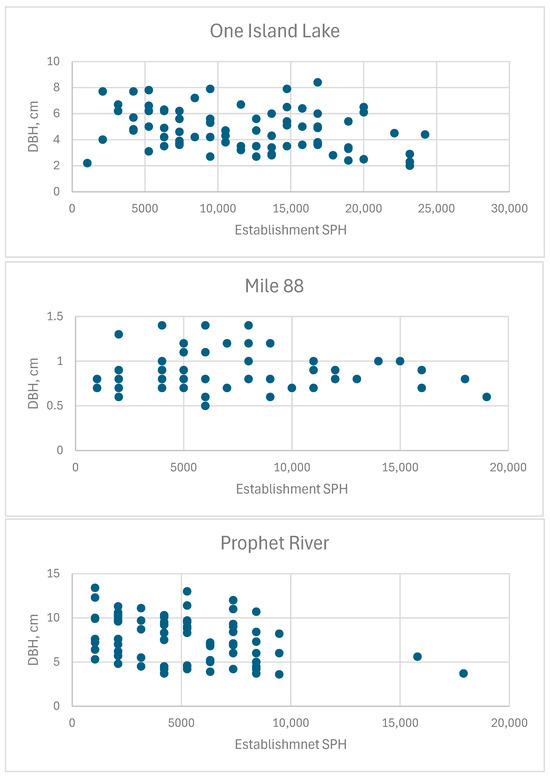
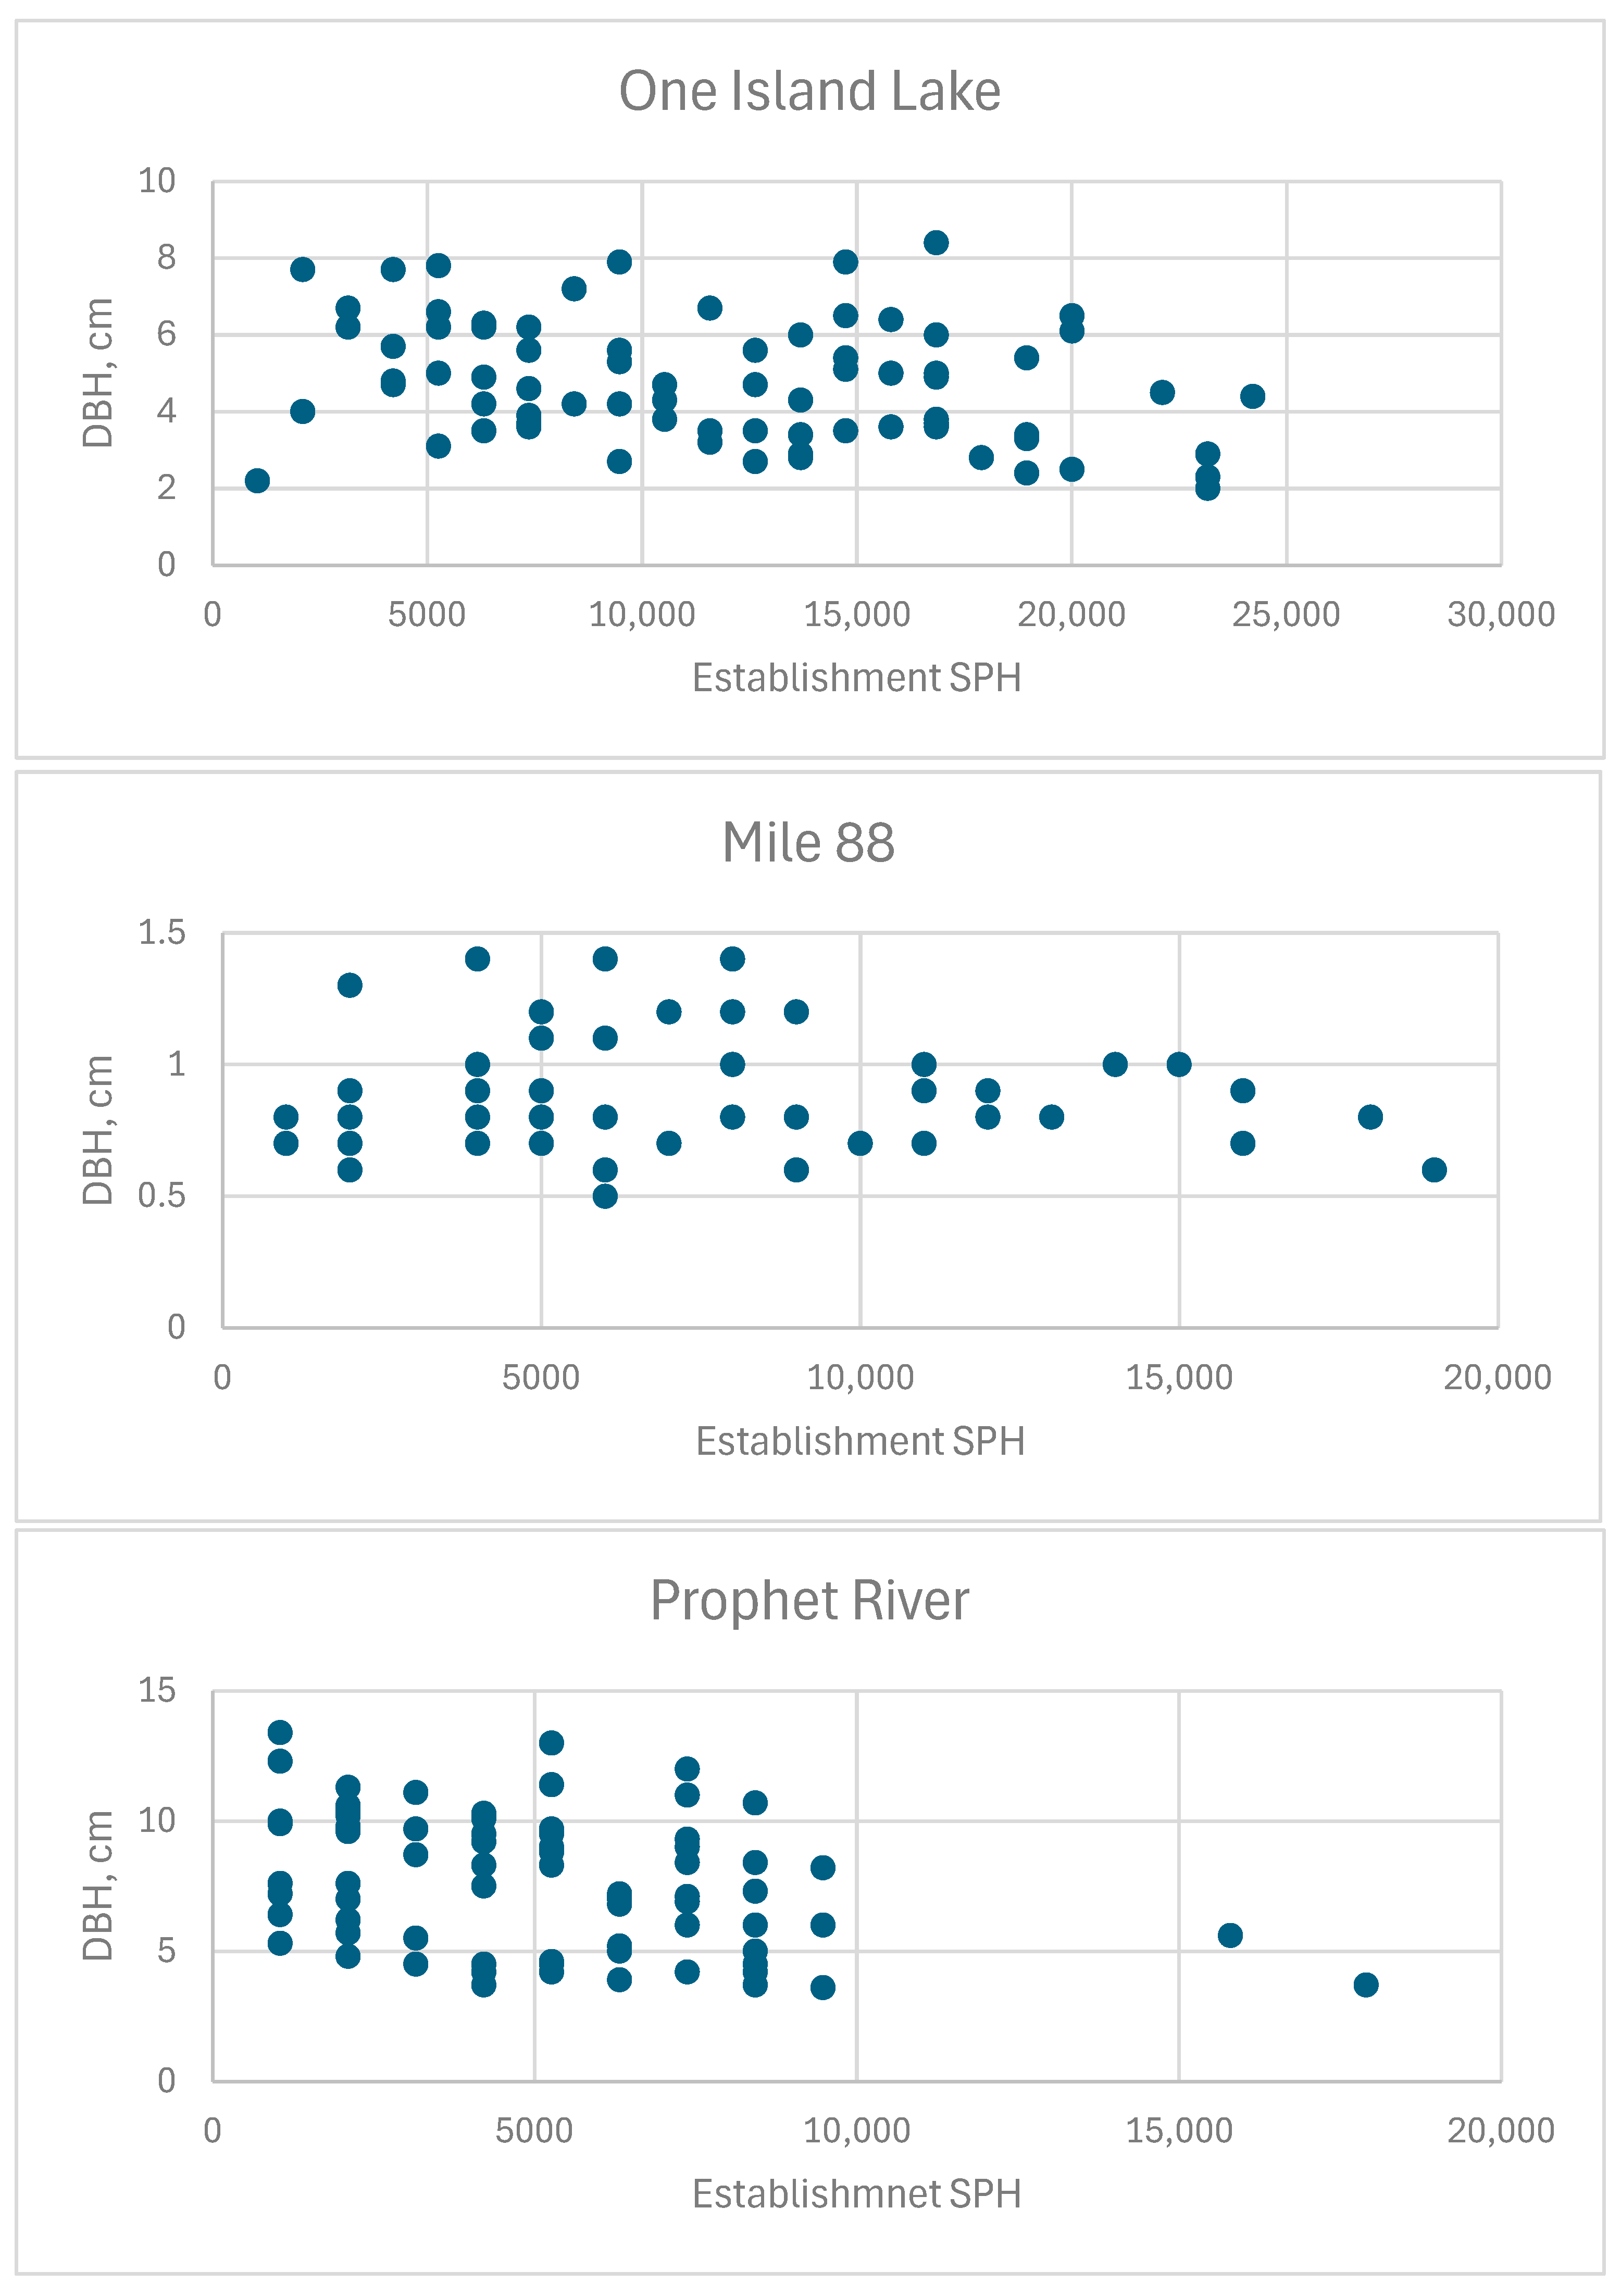
Competing species at One Island Lake and Mile 88 were similar: trembling aspen with minor amounts of balsam poplar (Populus balsamifera L.), lodgepole pine (Pinus contorta Dougl. Ex Loud. Var. latifolia Engelm.), black cottonwood (Populus trichocarpa Torr. & A. Gray), white spruce, and paper birch. Paper birch was the main crop tree competitor at the third site with aspen and white spruce being minor components. Stand density at trial establishment ranged respectively at One Island Lake, Mile 88, and Prophet River from 1000 (only the crop tree in the sample plot) to 23,000, 1000 to 34,000, and 1000 to 16,000. The mean density ± standard deviation at establishment for these sites was 10,232 (±5500), 8684 (±8801), and 3972 (±2808) respectively (Figure 1). Stand density for these sites at the last measure respectively were 7413 (±4483), 6204 (±4427), and 2986 (±2527). As stand density increased, crop tree DBH decreased at all sites (Figure 1).
Figure 1.
Crop tree DBH at establishment versus total establishment SPH at One Island Lake, Mile 88, and Prophet River.
Competitor mean height at establishment was greater than crop height at One Island Lake and Mile 88 but not at Prophet River (Table 2). Crop tree DBH was greater than that of competitors at One Island Lake and Prophet River but not at Mile 88 (Table 2). Competitors within 1 m critical FTG radius of the crop tree (not considered FTG) were the greatest at One Island Lake, intermediate at Mile 88, and lowest at Prophet River. Competing stem numbers (stems within 1 m of the crop tree) increased at Mile 88 (tree height < 1.3 m growing to height > 1.3 m and counted at second measurement) and decreased at other locations between the establishment and winter 2019–2020 measurements. The percentage of plots that were FTG at establishment was the greatest at Prophet River and the lowest at One Island Lake (Table 3). At two sites the number of FTG plots increased between measurements but at Mile 88 they decreased due to the noted recruitment (Table 3). None of the stands would be considered FTG by current BC criteria at either measurement.
Table 2.
Mean ± standard deviation (SD) crop tree and competition tree heights (HT, m), DBH (cm), and number of plots (n) at trial establishment at the three sites.
Table 3.
Percentage of plots that were FTG and not free-to-grow (NFTG) at trial establishment and after the 2019 growing season.
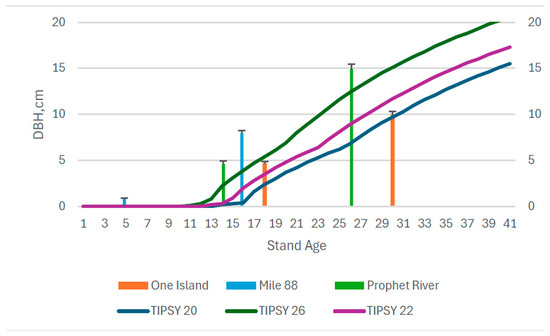
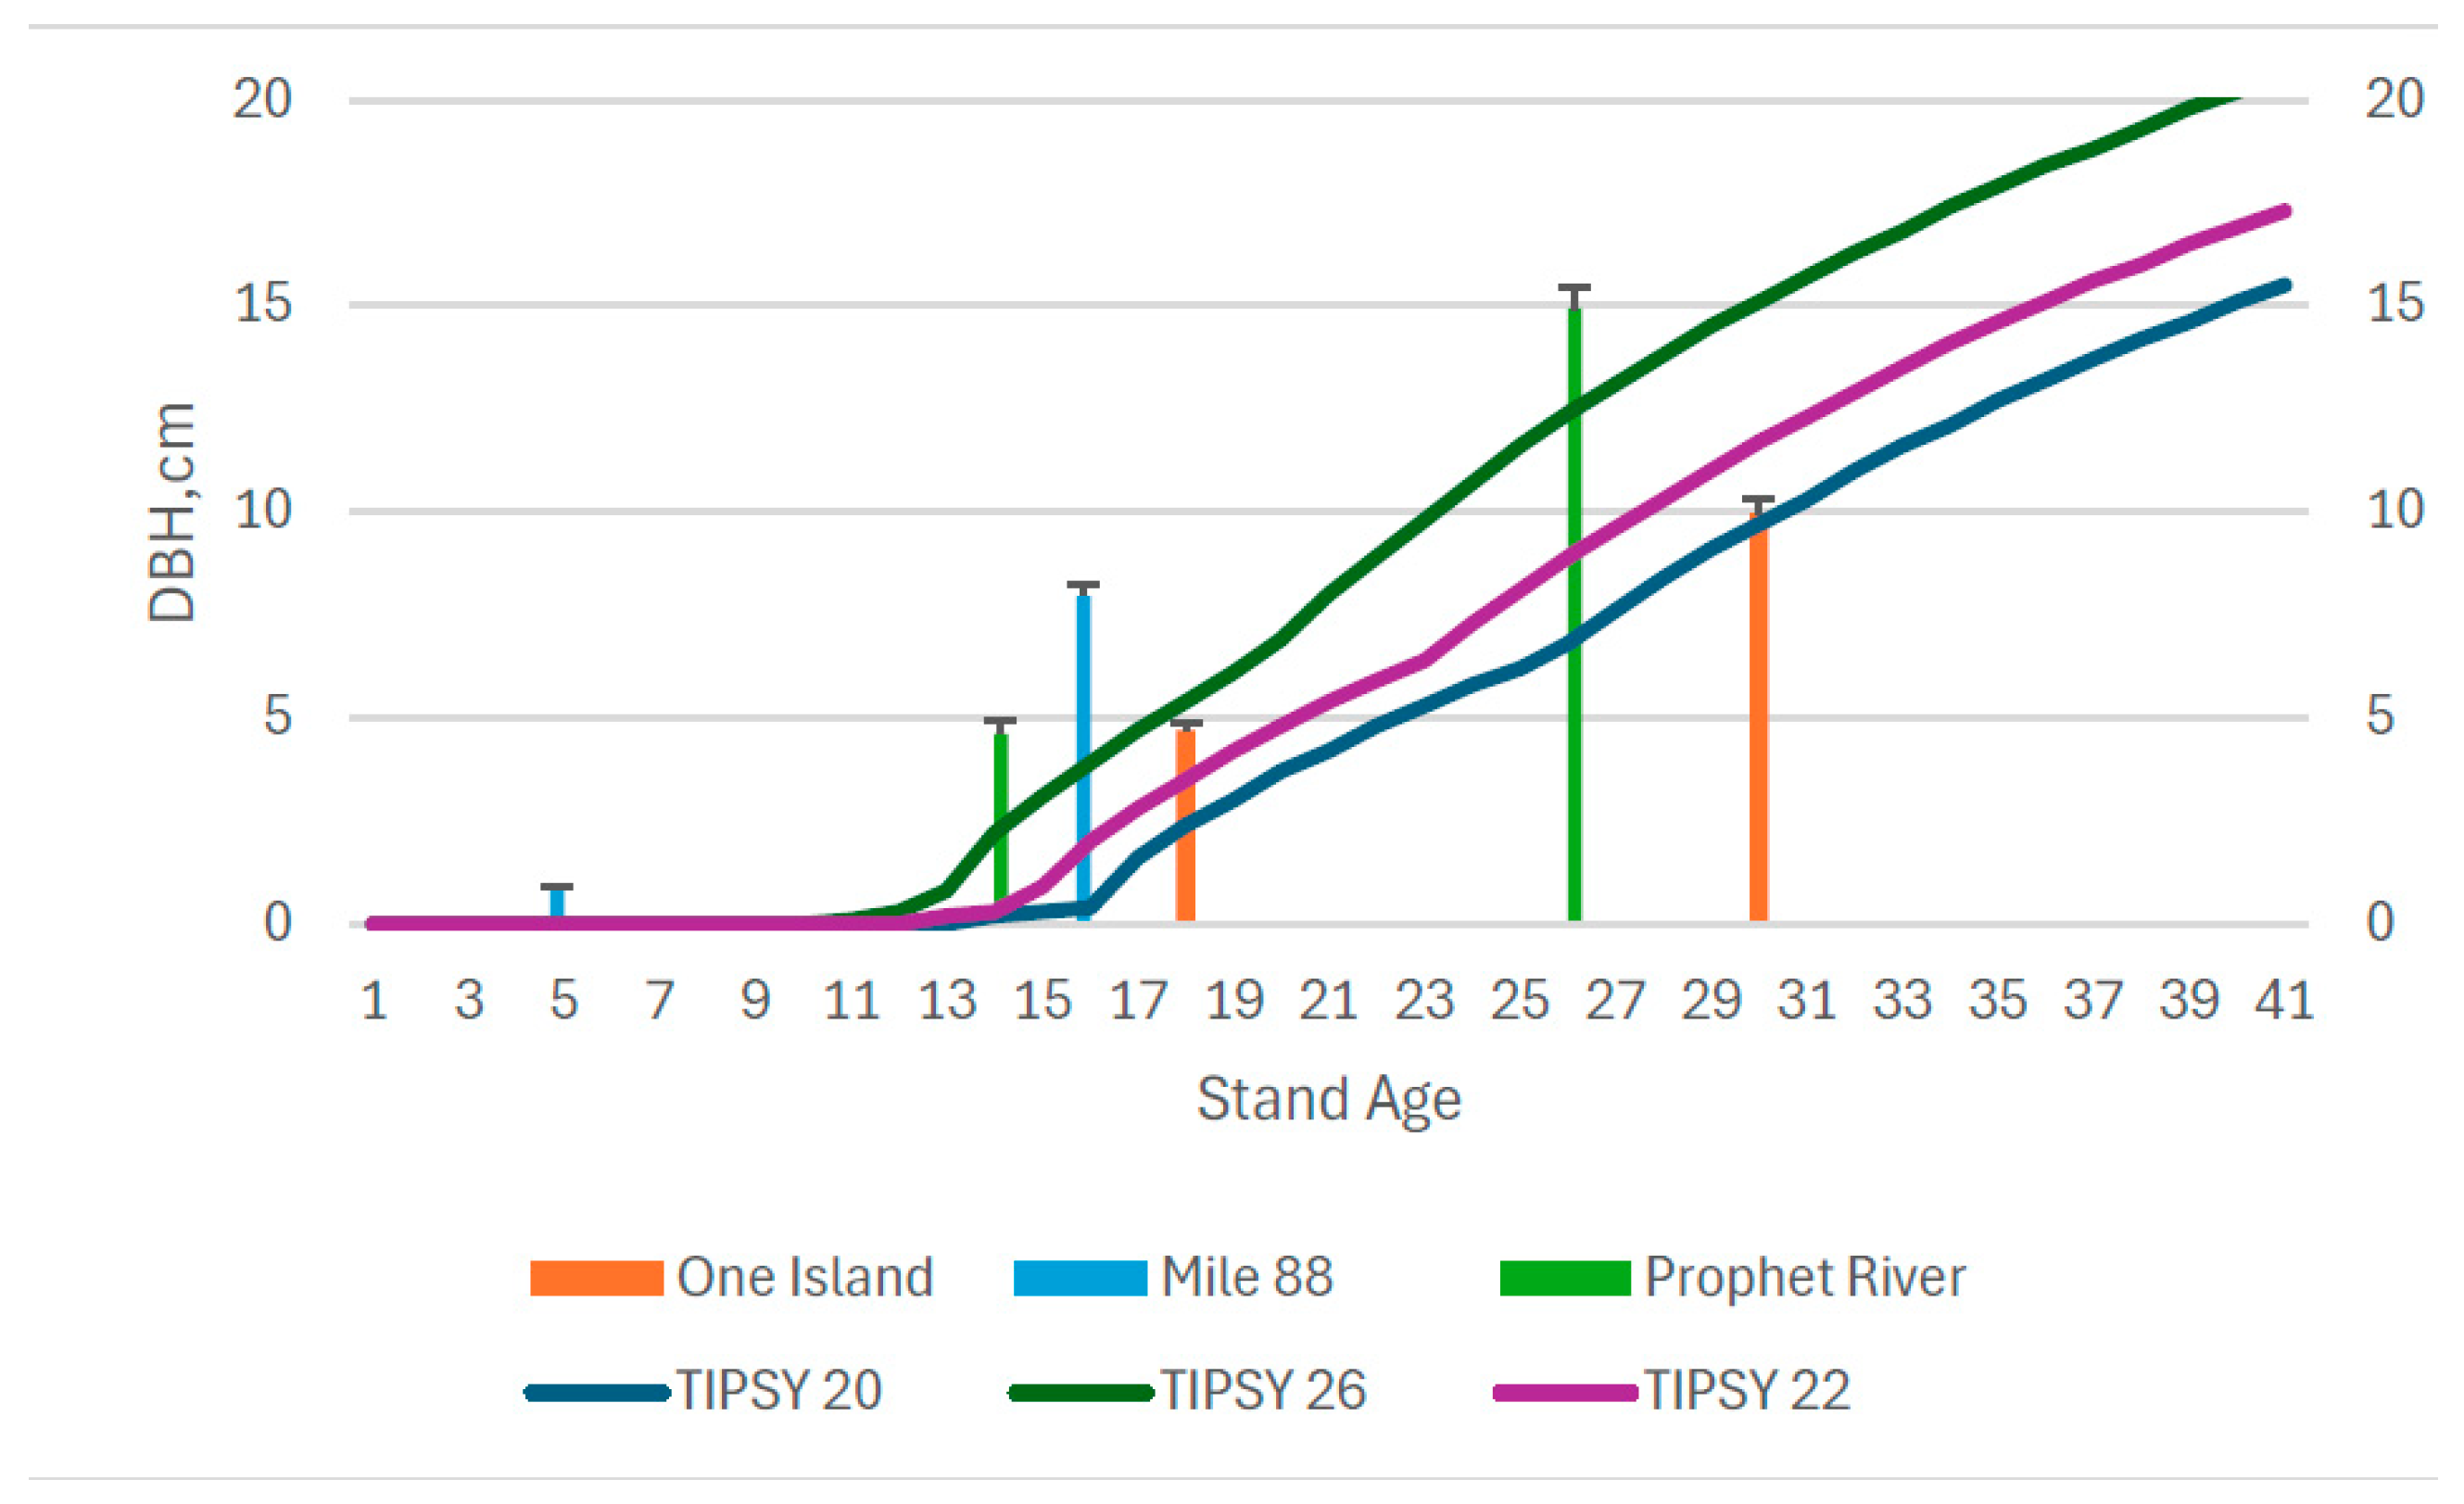
Mean DBH growth was greater in crop trees than in competing trees in all cases (Table 4). Competing trees had about twice the height growth of crop trees at One Island Lake and growth was similar at Mile 88. Height growth was not measured for competing trees at Prophet River. Mean crop tree DBH at all sites met or exceeded the DBH projection of TIPSY for the appropriate SI and stand age (Figure 2). At all sites, total mixedwood BA after the 2019 season was greater than the TIPSY projection and calculated spruce BA exceeded that projected by TIPSY (Table 5).
Table 4.
Mean ± standard deviation (SD) crop tree and competition tree heights (HT, m) and DBH (cm) growth from establishment to after the 2019 growing season at the three sites.
Figure 2.
Mean spruce crop tree DBH ± SEM for each site at trial establishment and after the 2019 growing season (bars), as well as the TIPSY DBH projections (curves) for sites of SI 20 (One Island Lake), SI 22 (Prophet River), and SI 26 (Mile 88).
Table 5.
Calculated basal area (BA) for spruce crop trees, spruce ingress, and broadleaves and TIPSY BA projection for spruce at the three sites after the 2019 season.
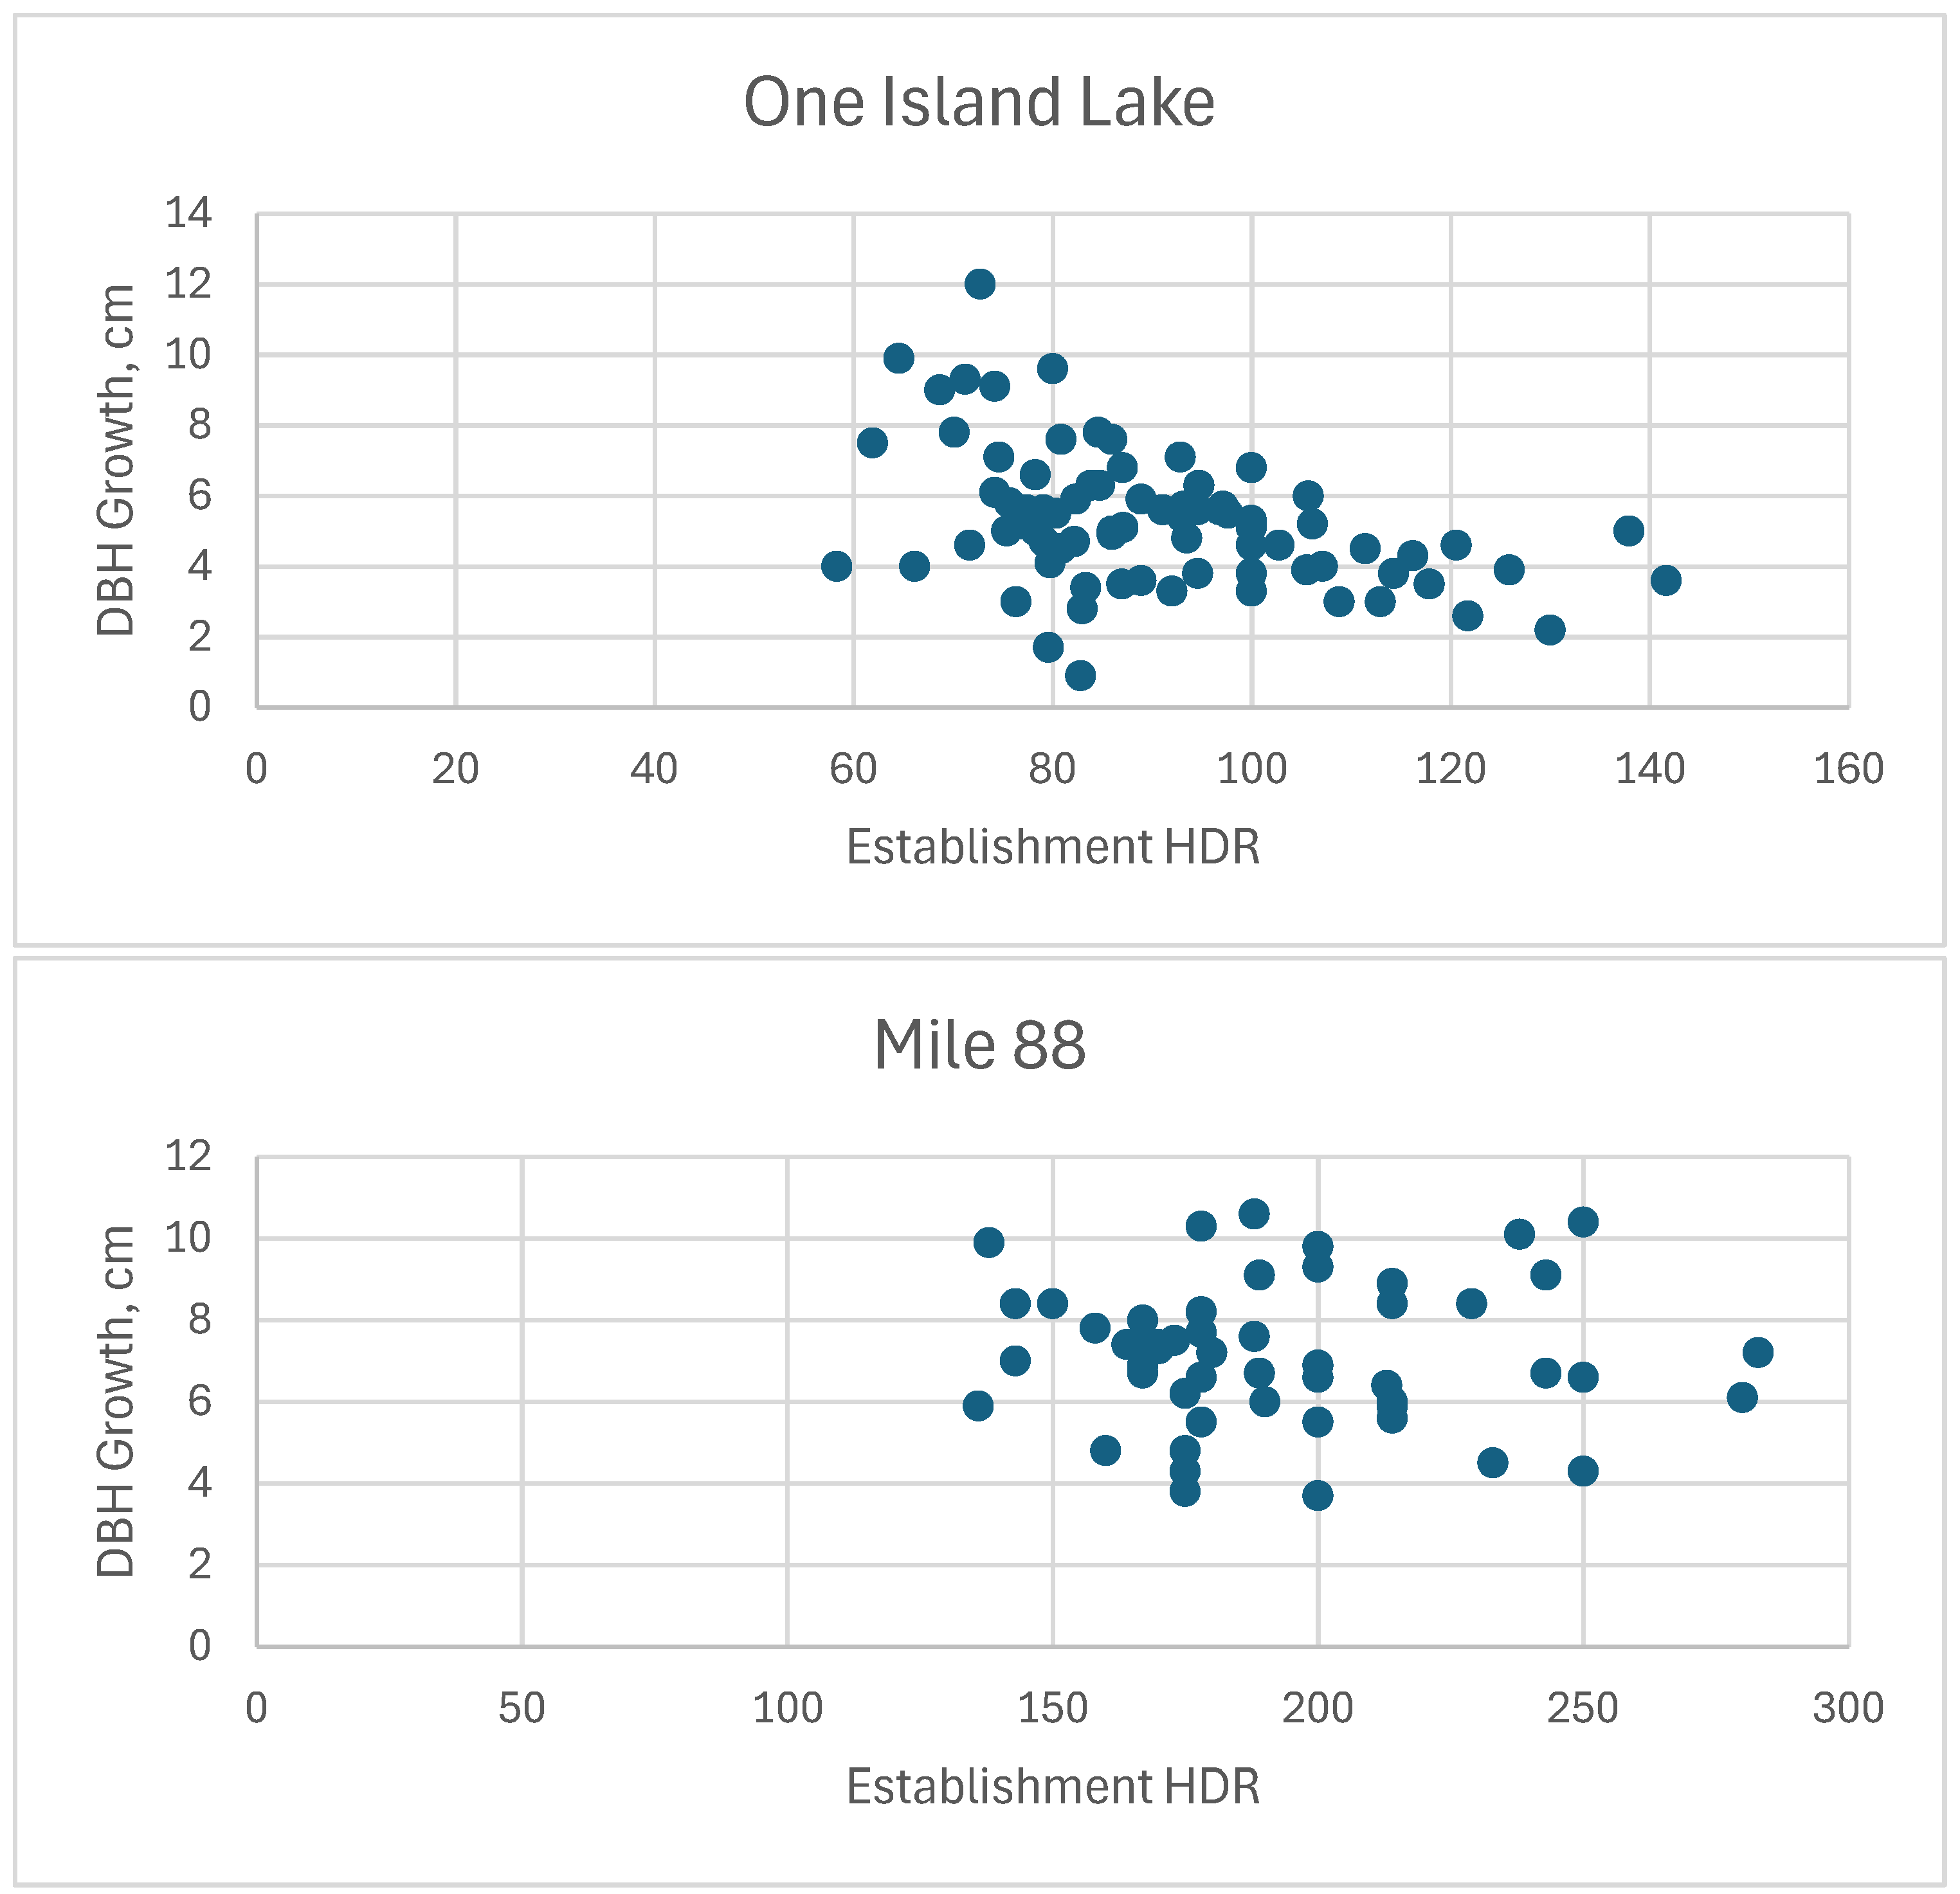
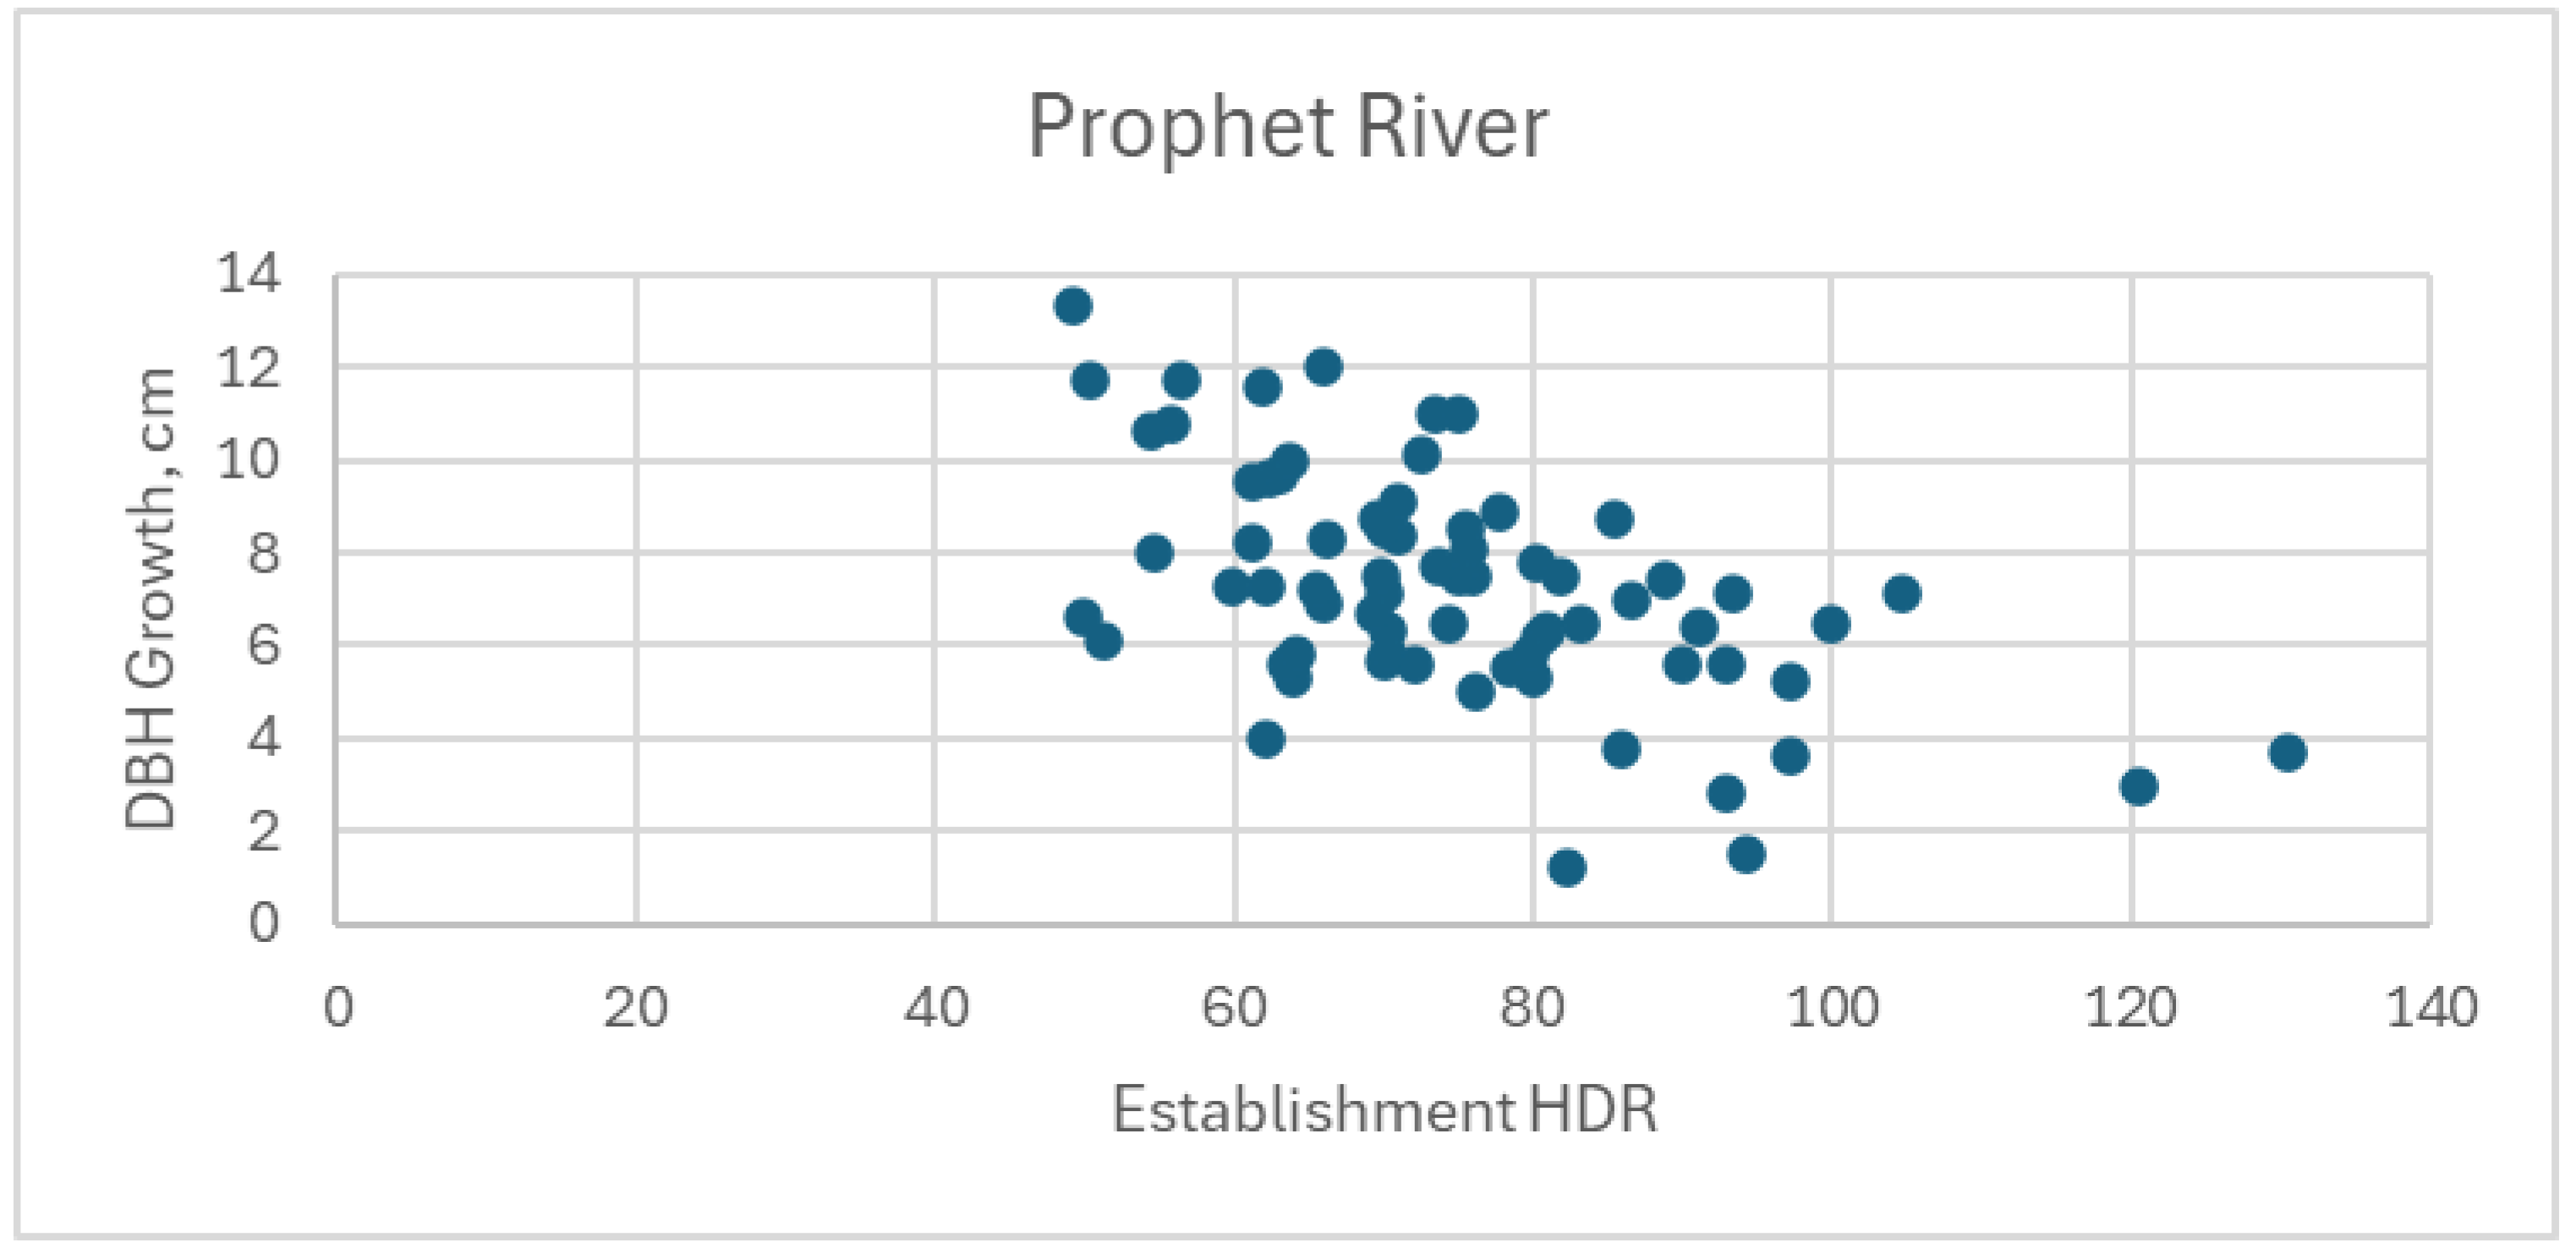
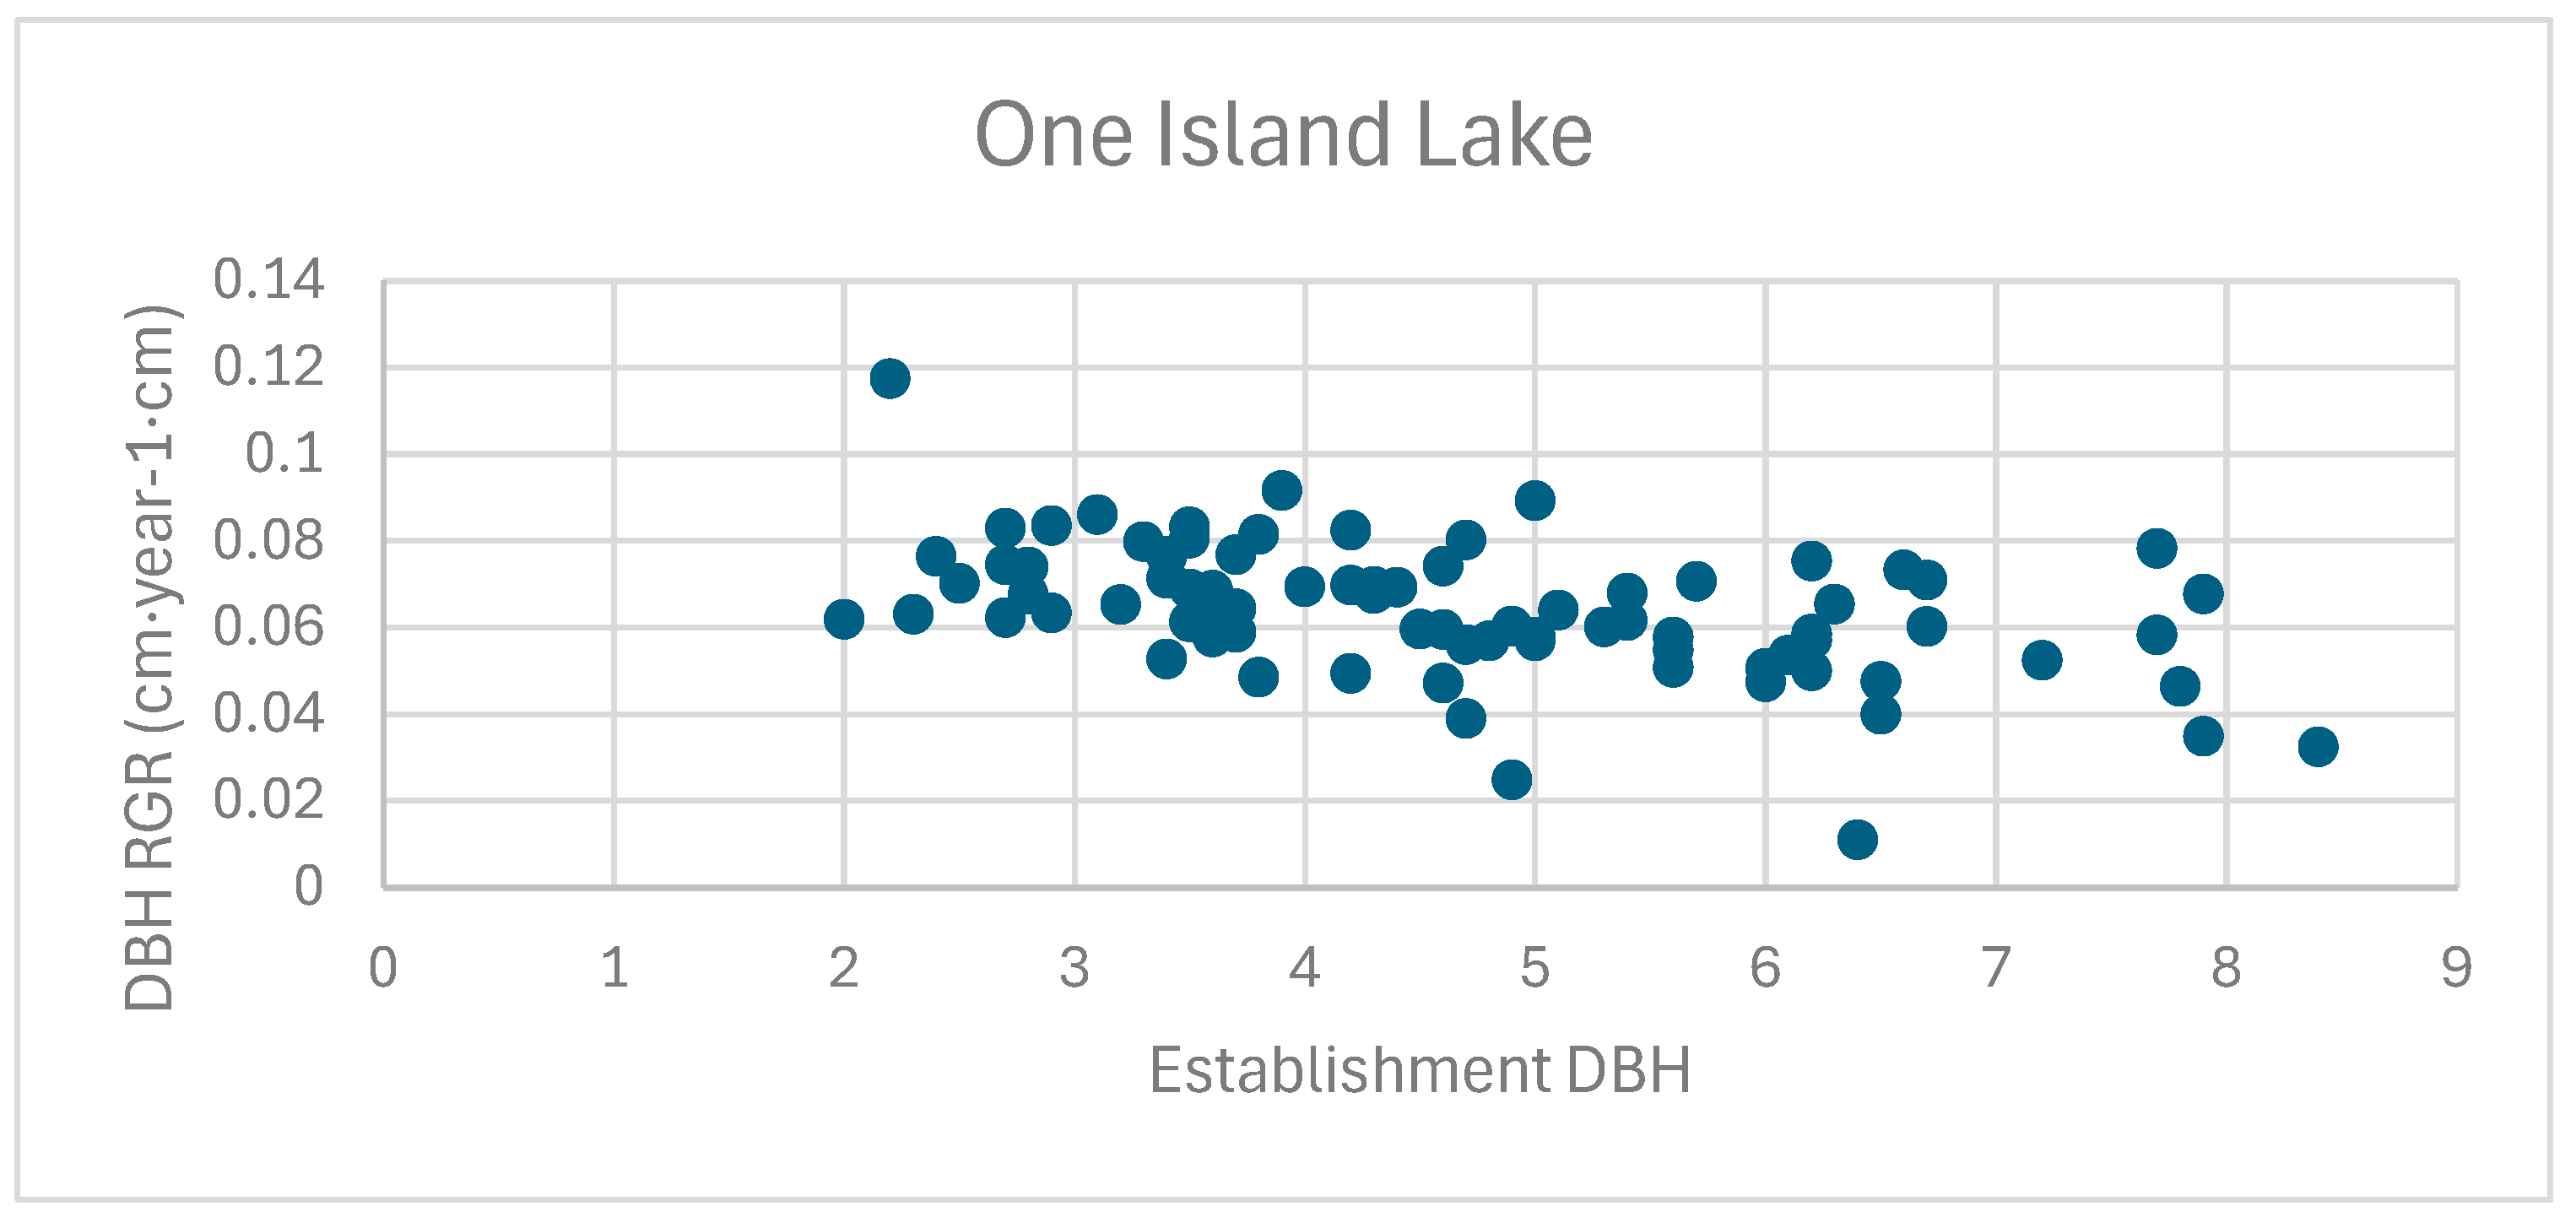
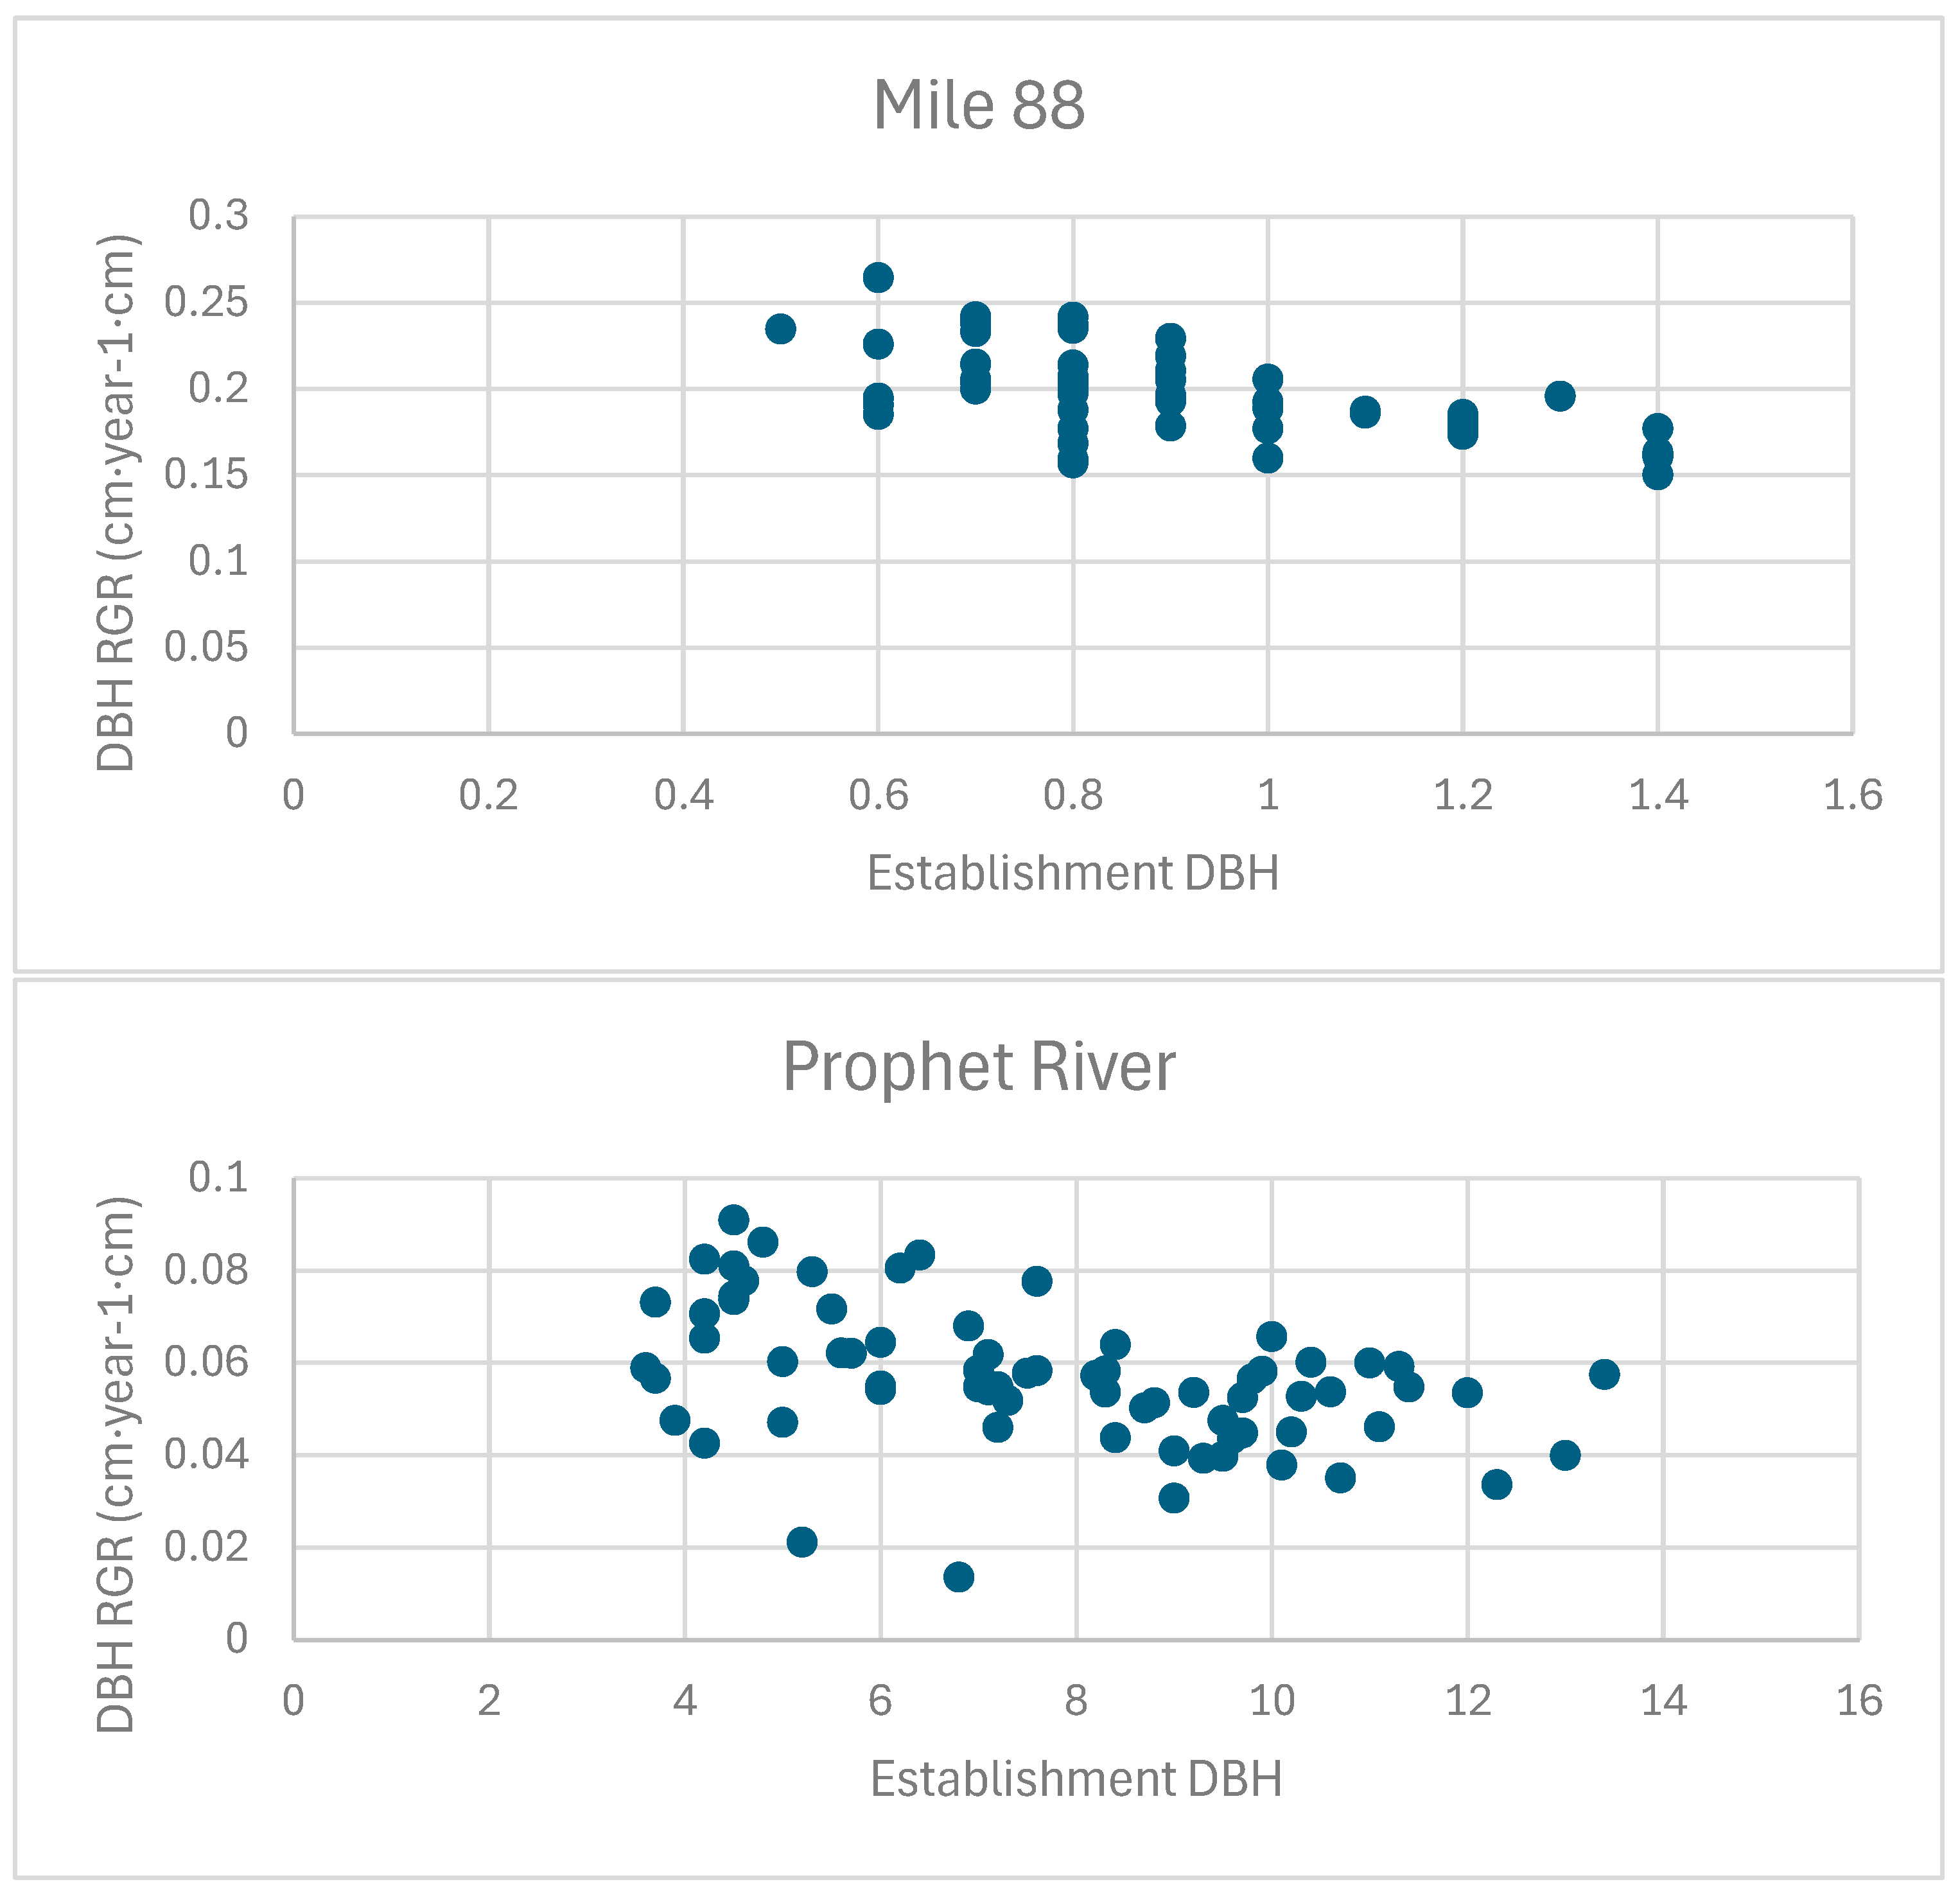
DBH growth decreased significantly (α = 0.05) as crop tree establishment HDR increased at the time of establishment at Prophet River and One Island Lake but there was no relationship for Mile 88 (Table 6 and Figure 3). The DBH RGR had a significant (α = 0.05) negative slope at all three sites with smaller DBH trees having greater growth rates than large trees (Table 6 and Figure 4). Mean crop tree DBH growth was greater than that of competitors at all sites (Table 4). The height relationship was not clear-cut (Table 4).
Table 6.
Regression of DBH growth versus HDR (DBH = constant + x × establishment HDR) at trial establishment and DBH RGR versus DBH (RGR = constant + x × establishment DBH) at trial establishment.
Figure 3.
Crop tree DBH growth versus establishment HDR at One Island Lake, Mile 88, and Prophet River.
Figure 4.
Mean DBH RGR versus crop tree establishment DBH at the three sites.
4. Discussion
4.1. Stand Stocking
Stand density decreased at One Island Lake and Prophet River between measurements as was predicted [28] and some aspen recruitment continued in the young stand at Mile 88. As expected [3,46,52,53,54], at trial establishment at the two older sites, competition negatively impacted crop tree DBH and if there was a density threshold, it exceeded 5000 SPH at all sites (Figure 1). This is much greater than the FTG threshold of 1000 SPH. However, at all sites mean crop tree DBH at establishment exceeded that projected by TIPSY (Figure 2). The SI values used in the TIPSY determination are greater than those that were obtained using SIBEC (site index by biogeoclimatic zone) [55], which is based on site nutrient and water relations. Therefore, if spruce DBH growth in the mixedwood exceeds that of the TIPSY projection, overall spruce DBH growth is not slowed by competing broadleaves. The model projection also indicated that there should be no measurable DBH at establishment for Mile 88. This leads to our questioning the applicability of current FTG standards for these sites. There was no apparent impact of broadleaf competition on crop tree establishment DBH at Mile 88 possibly due to young stand age, aspen co-establishing with spruce, spruce growing rapidly after planting, and it being of similar height at trial establishment. The establishment data and subsequent growth support observations that total growth can be greater in mixed-species stands without impacting conifer tree size [25,36,56,57] (Table 2 and Table 4). This suggests that species’ competitive interactions in mixedwoods (complex stands) may be different from those in pure stands [58].
4.2. Free-to-Grow
The FTG criteria in BC ignores the above possibility. Spruce, a mid seral species [47], developed below broadleaf trees in the boreal forest [11] under past ecological conditions but FTG criteria result in spruce stands and not mixedwoods. Today’s FTG criteria lead to stand simplification [4,11] and harm biodiversity [12,13]. As FTG criteria were originally developed for even-aged conifer stands [6,7], the disconnect is not unexpected. Therefore, current FTG standards are not relevant to sustainable management of boreal mixedwoods [59].
None of the stands could be considered FTG at either measurement (Table 3), yet DBH was greater than TIPSY projected for pure spruce stands of the same age at these sites. This may be due to intraspecific competition being greater in pure stands than interspecific competition in mixedwoods. The number of FTG plots did increase at two sites, by about 20 percent, and total broadleaf mortality increased at all sites but did not decrease within the 1 m radius at Mile 88 due to growth of trees too short to measure at establishment. Most of the plots at all sites exceeded the BC FTG standard maximum competitor density [6,7]. However, based on operational considerations and our findings, the broadleaves were not threatening future spruce growth at these sites as previously observed [1,2,3].
The FTG criteria fail to appreciate that mixedwoods promote greater stocking levels (Table 5) and maximum density [57] than pure stands [29], c.f., Figure 1. Hence their carrying capacity and productivity is greater [27,56]. Current FTG standards appear not to be related to mixedwood ecology [23,59,60] and forest management planning [9,11] and ignore their potential greater productivity, plus the associated non-timber resources, many of which are essential for Indigenous Treaty Rights.
4.3. Growth Metrics
The HDR indicated that slender trees were putting on less DBH growth than thicker trees (Table 6 and Figure 3), which is consistent with the observation that HDR is expected to increase with increased stand density or competition [61,62]. The DBH RGR had a significant negative slope at all sites (Table 6 and Figure 4) indicating broadleaf competition had not limited DBH growth [49,63] even though HDR indicates some impact. The impact of competition on target species can be estimated with RGR [64]. Larocque [65] suggested that DBH RGR was a preferred competition measure compared to absolute rate of growth. DBH RGR should increase with increased tree size (positive slope) if competition is a limiting factor but if it is not, DBH RGR should decrease (negative slope) with increased tree size [63,66] as demonstrated (Figure 4). This indicates that small trees are more efficient in stemwood production and not impacted by competition [50,63,66]. Unfortunately, DBH RGR is not a predictor of growth, but it is a result and has been previously noted that static indices have limited utility in predicting tree growth [67].
Mean crop tree DBH at both measurement periods exceeded or achieved the TIPSY pure stand projection at all sites of appropriate age and productivity (Figure 2; Table 2, Table 4 and Table 5). Also, the total BA (Table 5) is several times greater than the BA projected for a pure spruce stand of the same age indicating much greater productivity and carrying capacity in a mixedwood stand [27,57]. These mixedwoods have much greater total productivity than a pure spruce stand growing on the same BEC unit (Figure 2, SI plots). This has been demonstrated by many [25,68,69,70,71] but there are contradictory findings too, generally in older work [17,18,20,21]. Measured spruce BA is also greater than the TIPSY projection (Table 5) and is mainly in the larger DBH classes suggesting that broadleaves have not negatively impacted spruce growth. Also, the BA (Table 5) may indicate that birch is a weaker competitor than aspen [70], as shown between One Island Lake and Prophet River, but Stadt et al. [71] suggest the opposite. The species’ response may be site-specific.
Facilitation or complementarity between species probably accounts for increased productivity [25]. Specific to the boreal forest in western Canada, the more rapid decomposition of broadleaf leaf litter [72,73] and quality nutrient acquisition [67] likely benefit spruce. Similar conifer growth in mixed stands plus the added growth of broadleaves has been reported in Scandinavia [74]. The connection between the FTG criteria, stand stocking, and mixedwood growth is clearly lacking [1,2,9,75].
4.4. Operational Considerations
Our observations argue against broadcast removal of competing broadleaf species [4,76] at similar spruce mixedwood sites. Broadcast removal appears not to enhance tree growth [2], but it eliminates the mixedwoods’ ecological goods and services [12,14,33,34]. There is also the extra cost of competitor removal. This suggests that the BC Government’s FTG (reforestation performance) criteria are not biologically based as competition levels at all three sites far exceeded the FTG’s usual standard maximum competition density threshold [6]. Several reports indicated that for conifers classed as FTG or not FTG at trial establishment, there was no significant difference in DBH or height growth after a decade [1,9,75]. This is not implying that there is not a competition level or species composition in mixedwoods that reduces crop tree growth below an acceptable operational minimum. However currently in BC, we do not have an agreed-upon administrative threshold or protocols to define one for mixedwoods in northeast BC [59].
Competition should reduce growth efficiency of small trees more than that of the large ones [66] but our findings do not support this and counter the present management tactic to remove competition with a broadcast brushing treatment. Not brushing may have a positive economic impact [3] and it definitely has positive ecological [12] and societal [14] impacts. The accepted negative impact of retaining broadleaves regionally is related to their low value due to weak or lack of commercial markets [77,78]. However, this view does not consider the removal cost, lost productivity, or lost ecological values if sites are brushed [4]. It has been suggested that mixedwoods in the longer term may significantly reduce financial risk due to accrued ecological benefits [79] and their hypothesized ability to better respond to a changing climate [44,45]. As importantly as the preceding (or even more importantly), BC First Nations currently view the use of chemical brushing and loss of habitat as a major forest management shortfall [14,15,80]. Mixedwood management (retaining broadleaves) can start addressing their concern.
When competition is limiting tree growth, perhaps spot removal of undesirable levels of competing vegetation around individual crop trees is a sensible economic–ecological–social compromise [3]. However, doing no competition control at sites like these may be a reasonable approach as stand growth has not been compromised even though growth of some individual trees may have been. The latter is based on our data indicating that overall stand level spruce growth was not significantly impacted by high levels of broadleaf competition. The proposed protocol would be difficult to implement operationally as our metrics are not predictive. Tree DBH could be sampled and if the stand result is as good as the TIPSY projection, then no broadleaf brushing will be needed. Clearly more data is needed to bring the approach to an operational level. In the first instance, our approach is only for spruce–broadleaf mixtures as it has yet to be demonstrated for lodgepole pine mixedwoods in northeast BC (c.f., Harper [53,54]).
5. Conclusions
Spruce DBH growth in broadleaf mixtures was as good as or superior to projections for pure spruce stands in northeast BC of appropriate documented site productivity (SI) and age. Retaining mixedwoods at the sites we examined shows that overall conifer productivity has not been impaired; in fact, total site productivity is increased, and the ecological and social benefits associated with mixedwoods are retained or possibly enhanced. Our observations reinforce the suggestion that broadleaf stand components should not only be viewed as tolerable but often as beneficial [81]. However, these data do not aid our management dilemma—how to identify mixedwood stands that will or will not meet legislated conifer growth expectations (targets) for managers. On the other hand, perhaps forest management should focus on desired future forest values, in line with traditional First Nations world view, rather than short-term timber product volume expectations on a rotation of about 80 years. A sustained market for broadleaves would help meet industry and government objectives and support Indigenous traditions.
Author Contributions
Conceptualization, C.H., C.M. and J.B.; methodology, C.H.; formal analysis, C.H.; resources, C.M. and J.B.; data collection, C.M., J.B. and C.H.; data curation, C.H.; writing—original draft preparation, C.H.; writing—review and editing, C.M., J.B. and C.H.; supervision, C.H.; project administration, C.M.; funding acquisition, J.B., C.M. and C.H. All authors have read and agreed to the published version of the manuscript.
Funding
Support for site remeasurement was provided by the Association of Peace River Woodlots and the BC Wood Products Development Council. Trial establishment was done while the lead author held the FRBC—Slocan Mixedwood Chair at the University of Northern British Columbia and it was funded by the British Columbia Forest Science Program.
Data Availability Statement
The lead author should be contacted for data requests.
Acknowledgments
The efforts of Nicole Balliet, Kyle Runzer, Cindy Baker and Eduardo Bittencourt who established these sites under trying conditions is recognized. The reviewers’ comments helped improve the manuscript.
Conflicts of Interest
The authors declare no conflicts of interest.
References
- Dhar, A.; Wang, J.R.; Hawkins, C.D.B. Interaction of trembling aspen and lodgepole pine in a young sub-boreal mixedwood stand in Central British Columbia. Open J. For. 2015, 5, 129. [Google Scholar] [CrossRef]
- Hawkins, C.; Maundrell, C. Linking silvics to policy: A disconnect with free-to-grow standards in northeast British Columbia. Forests 2026, 17, 21. [Google Scholar] [CrossRef] [Scilit]
- Hawkins, C.D.B.; Dhar, A.; Rogers, B.J. How much birch (Betula papyrifera) is too much for maximizing spruce (Picea glauca) growth: A case study in boreal spruce plantation forests. J. For. Sci. 2012, 58, 314–327. [Google Scholar] [CrossRef] [Scilit]
- Simard, S.W.; Vyse, A. Trade-offs between competition and facilitation: A case study of vegetation management in the interior cedar-hemlock forests of southern British Columbia. Can. J. For. Res. 2006, 36, 2486–2496. [Google Scholar] [CrossRef] [Scilit]
- Knoke, T.; Stimm, B.; Ammer, C.; Moog, M. Mixed forests reconsidered: A forest economics contribution on an ecological concept. For. Ecol. Manag. 2005, 213, 102–116. [Google Scholar] [CrossRef] [Scilit]
- BC Ministry of Forests. Establishment to Free Growing Guidebook, Prince George Forest Region, Ver 2.3; BC Ministries of Forests and Environment: Victoria, BC, Canada, 2000; pp. 24–39. [Google Scholar]
- British Columbia (BC) Ministry of Forests. Reference Guide for Forest Development Stocking Standards. 2021. Available online: https://www2.gov.bc.ca/gov/content/industry/forestry/managing-our-forest-resources/silviculture/stocking-standards?keyword=2021 (accessed on 9 April 2026).
- Armson, K.A. Regeneration standards: What has the past to show us? For. Chron. 2005, 81, 781–784. [Google Scholar] [CrossRef] [Scilit]
- Lieffers, V.J.; Stadt, K.J.; Feng, Z. Free-to grow regeneration standards are poorly linked to growth of spruce in boreal mixedwoods. For. Chron. 2007, 83, 818–824. [Google Scholar] [CrossRef] [Scilit]
- Farnden, C. Development of Regeneration Standards for Sustainable Forest Management. Ph.D. Thesis, University of British Columbia, Vancouver, BC, Canada, 2010. [Google Scholar]
- Lieffers, V.J.; Armstrong, G.W.; Stadt, K.J.; Marenholtz, E.H. Forest regeneration standards: Are they limiting management options for Alberta’s boreal mixedwoods? For. Chron. 2008, 84, 76–82. [Google Scholar] [CrossRef] [Scilit]
- Chen, S.; Shahi, C.; Chen, H.Y.H.; Kumar, P.; Ma, Z.; McLaren, B. Trade-offs and synergies between economic gains and plant diversity across a range of management alternatives in boreal forests. Ecol. Econ. 2018, 151, 162–172. [Google Scholar] [CrossRef] [Scilit]
- Eggers, J.; Lundström, J.; Snäll, T.; Öhman, K. Balancing wood production and biodiversity in intensively managed boreal forest. Scand. J. For. Res. 2022, 37, 213–225. [Google Scholar] [CrossRef] [Scilit]
- Kayahara, G.J.; Armstrong, C.L. Understanding First Nations rights and perspectives on the use of herbicides in forestry: A case study from northeastern Ontario. For. Chron. 2015, 91, 126–140. [Google Scholar] [CrossRef] [Scilit]
- BCFNGC and PBC (British Columbia First Nations Forestry Council and Province of British Columbia). BC First Nations Forestry Strategy. 2019. Available online: https://www.bcafn.ca/sites/default/files/docs/resolutions/2019_26_AGM_Resolution_DevelopmentandImplementationofBCForestStrategy.pdf (accessed on 10 April 2026).
- Tarrant, R.; Trappe, J. The role of Alnus in improving the forest environment. Plant Soil. 1971, 19, 335–348. [Google Scholar] [CrossRef] [Scilit]
- Binkley, D. Ecosystem production in Douglas-fir plantations: Interaction of red alder and site fertility. For. Ecol. Manag. 1983, 5, 215–227. [Google Scholar] [CrossRef] [Scilit]
- Frivold, L.; Mielikainen, K. The effects of hardwoods on softwood growth in mixed stands in Fennoscandia. In The Silvics and Ecology of Boreal Spruces; Titus, B.D., Lavigne, M.B., Newton, P.F., Meades, W.J., Eds.; IUFRO Working PartySI.05-12 Symposium Proceedings, 12–17 August 1989, Information Report Number N-X-271; Forestry Canada Newfoundland Forestry Centre: Corner Brook, NL, Canada, 1990; pp. 75–82. [Google Scholar]
- Binkley, D. Mixtures of nitrogen fixing tree species. In The Ecology of Mixed Species Stands of Trees; Cannell, M.G.R., Malcolm, D.C., Robertson, P.A., Eds.; British Ecological Society Special Publication 11; Blackwell Scientific Publications: Oxford, UK, 1992; pp. 99–123. [Google Scholar]
- Kelty, M.J. Comparative productivity of monocultures and mixed-species stands. In The Ecology and Silviculture of Mixed Species Forests; Kelty, M.J., Larson, B.C., Oliver, C.D., Eds.; Kluwer Academic Publishers: Dordrescht, The Netherlands, 1992; pp. 125–141. [Google Scholar]
- Mårda, H. The influence of a birch shelter (Betula spp.) on the growth of young stands of Picea abies. Scand. J. For. Res. 1996, 11, 343–350. [Google Scholar] [CrossRef] [Scilit]
- Dudelis, J. Development of Stratified Spruce-Birch Stands in Latvia. Master’s Thesis, Swedish University of Agricultural Sciences, Umea, Sweden, 2013; 64p. Available online: https://stud.epsilon.slu.se/5846/7/dudelis_j_130704.pdf (accessed on 9 April 2026).
- Man, R.; Lieffers, V.J. Are Mixtures of Aspen and White Spruce More Productive than Single Species Stands? For. Chron. 1999, 75, 505–513. [Google Scholar] [CrossRef] [Scilit]
- Simard, S.W.; Hagerman, S.M.; Sachs, D.L.; Heineman, J.L.; Mather, W.J. Conifer growth, Armillaria ostoyae root disease and plant diversity responses to broadleaf competition reduction in temperate mixed forests of southern interior British Columbia. Can. J. For. Res. 2005, 35, 843–859. [Google Scholar] [CrossRef] [Scilit]
- Kelty, M.J. The role of species mixtures in plantation forestry. For. Ecol. Manag. 2006, 233, 195–204. [Google Scholar] [CrossRef] [Scilit]
- Pretzsch, H.; Schutze, G. Transgressive overyielding in mixed compared with pure stands of Norway spruce and European beech in Central Europe: Evidence on stand level and explanation on individual tree level. Eur. J. For. Res. 2009, 128, 183–204. [Google Scholar] [CrossRef] [Scilit]
- Pretzsch, H.; Schutze, G. Effect of tree species mixing on the size structure, density, and yield of forest stands. Eur. J. For. Res. 2016, 135, 1–22. [Google Scholar] [CrossRef] [Scilit]
- Kabzems, R.D.; Bokalo, M.; Comeau, P.G.; MacIsaac, D.A. Managed mixtures of aspen and white spruce 21 to 25 years after establishment. Forests 2016, 7, 5. [Google Scholar] [CrossRef] [Scilit]
- Kweon, D.; Comeau, P.G. Factors influencing overyielding in young boreal mixedwood stands in western Canada. For. Ecol. Manag. 2019, 432, 546–557. [Google Scholar] [CrossRef] [Scilit]
- Elgie, S.; McCarney, G.R.; Adamowicz, W.L. Assessing the implications of a carbon market for boreal forest management. For. Chron. 2011, 87, 367–381. [Google Scholar] [CrossRef] [Scilit]
- Taylor, A.R.; Seedre, M.; Brassard, B.W.; Chen, H.Y. Decline in net ecosystem productivity following canopy transition to late-succession forests. Ecosystems 2014, 17, 778–791. [Google Scholar] [CrossRef] [Scilit]
- Payne, N.J.; Cameron, D.A.; Leblanc, I.-D.; Morrison, I.K. Carbon storage and net primary productivity in Canadian boreal mixedwood stands. J. For. Res. 2019, 30, 1667–1678. [Google Scholar] [CrossRef] [Scilit]
- Aldea, J.; Bravo, F.; Vazquez-Piqu, J.; Ruíz-Peinado, R.; del Río, M. Differences in stem radial variation between Pinus pinaster Ait. and Quercus pyrenaica Willd. may release inter-specific competition. For. Ecol. Manag. 2021, 481, 118779. [Google Scholar] [CrossRef] [Scilit]
- Piotto, D. A meta-analysis comparing tree growth in monocultures and mixed plantations. For. Ecol. Manag. 2008, 255, 781–786. [Google Scholar] [CrossRef] [Scilit]
- Felton, A.; Nilsson, U.; Sonesson, J.; Felton, A.M.; Roberge, J.-M.; Ranius, T.; Ahlström, M.; Bergh, J.; Björkman, C.; Boberg, J.; et al. Replacing monocultures with mixed-species stands: Ecosystem service implications of two production forest alternatives in Sweden. Ambio 2016, 45, S124–S139. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jactel, H.; Gritti, E.S.; Drössler, L.; Forrester, D.I.; Mason, W.L.; Morin, X.; Pretzsch, H.; Castagneyrol, B. Positive biodiversity–productivity relationships in forests: Climate matters. Biol. Lett. 2018, 14, 20170747. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Eastman, D.S. Habitat Selection and Use in Winter by Moose in Sub-Boreal Forests of North-Central British Columbia, and Relationships to Forestry. Ph.D. Thesis, University of British Columbia, Vancouver, BC, Canada, 1977; 554p. Available online: http://hdl.handle.net/2429/21531 (accessed on 10 April 2026).
- Hobson, K.A.; Bayne, E. Breeding bird communities in boreal forest of Western Canada: Consequences of “Unmixing” the mixedwoods. Condor 2000, 102, 759–769. [Google Scholar]
- Cavard, X.; Macdonald, S.E.; Bergeron, Y.; Chen, H.Y.H. Importance of mixedwoods for biodiversity conservation: Evidence for understory plants, songbirds, soil fauna, and ectomycorrhiza in northern forests. Environ. Rev. 2011, 19, 142–161. [Google Scholar] [CrossRef] [Scilit]
- Fraser Basin Council. Climate Projections for the BC Northeast Region; Fraser Basin Council: Vancouver, BC, Canada, 2019; p. 45. Available online: https://www.fraserbasin.bc.ca/_Library/CCAQ/fbc_ne_climatereport_web.pdf (accessed on 10 April 2026).
- Halim, M.A.; Chen, H.Y.H.; Thomas, S.C. Stand age and species composition effects on surface albedo in a mixedwood boreal forest. Biogeosciences 2019, 16, 4357–4375. [Google Scholar] [CrossRef] [Scilit]
- Oboite, F.O.; Comeau, P.G. The interactive effect of competition and climate on growth of boreal tree species in western Canada and Alaska. Can. J. For. Res. 2020, 50, 457–464. [Google Scholar] [CrossRef] [Scilit]
- Hamann, A.; Wang, T. Potential effects of climate change on ecosystem and tree species distribution in British Columbia. Ecology 2006, 87, 2772–2786. [Google Scholar] [CrossRef] [Scilit]
- Boulanger, Y.; Taylor, A.R.; Price, D.T.; Cyr, D.; McGarrigle, E.; Rammer, W.; Sainte-Marie, G.; Beaudoin, A.; Guindon, L.; Mansuy, N. Climate change impacts on forest landscapes along the Canadian southern boreal forest transition zone. Landsc. Ecol. 2017, 32, 1415–1431. [Google Scholar] [CrossRef] [Scilit]
- DeLong, S.C.; Banner, A.; MacKenzie, W.H.; Rogers, B.J.; Kaytor, B. A Field Guide to Ecosystem Identification for the Boreal White and Black Spruce Zone of British Columbia; Land Management Handbook 65; BC Ministry of Forests and Range: Victoria, BC, Canada, 2011. Available online: www.for.gov.bc.ca/hfd/pubs/Docs/Lmh/Lmh65.htm (accessed on 6 April 2026).
- Jiang, X.; Huang, J.G.; Stadt, K.J.; Comeau, P.G.; Chen, H.Y.H. Spatial climate-dependent growth response of boreal mixedwood forest in western Canada. Glob. Planet. Change 2016, 139, 141–150. [Google Scholar] [CrossRef] [Scilit]
- Nienstaedt, H.; Zasada, J.C. Picea glauca (Moench) Voss—White spruce. In Silvics of North America, Volume 1: Conifers; Burns, R.M., Hankala, B.H., Coord.; USDA Forest Service Agriculture Handbook 654; United States Department of Agriculture (USDA): Washington, DC, USA, 1990; pp. 204–226. [Google Scholar]
- Kent, M.; Coker, P. Vegetation Description and Analysis: A Practical Approach; CRC Press: Boca Raton, FL, USA, 1992. [Google Scholar]
- Hunt, R. Plant Growth Analysis, 2nd ed.; Natural Environment Research Council: London, UK, 1982; pp. 5–41. [Google Scholar]
- Nigh, G.D. Growth Intercept Models and Tables for British Columbia: Interior Species, 3rd ed.; Land Management Handbook Field Guide Insert 10; BC Ministry of Forests, Research Branch: Victoria, BC, Canada, 1999. Available online: https://www.for.gov.bc.ca/hfd/pubs/Docs/Fgi/Fgi10-files/fgi10-r3.pdf (accessed on 1 April 2026).
- Mission, L.; Vincke, C.; Devillez, F. Frequency responses of radial growth series after different thinning intensities in Norway spruce (Picea abies (L.) Karst.) stand. For. Ecol. Manag. 2003, 177, 51–63. [Google Scholar] [CrossRef] [Scilit]
- Oliver, C.D.; Larson, B.C. Forest Stand Dynamics; John Wiley and Sons: New York, NY, USA, 1996; pp. 41–88. [Google Scholar]
- Harper, G. Lodgepole pine and trembling aspen mixedwoods: Growth and yield within 22 to 39-year-old pine plantations of northern interior British Columbia. For. Chron. 2015, 91, 502–518. [Google Scholar] [CrossRef] [Scilit]
- Harper, G. Lodgepole pine and trembling aspen competition: Neighbourhood studies within 22 to 39-year-old pine plantations of northern British Columbia. For. Chron. 2017, 93, 226–240. [Google Scholar] [CrossRef] [Scilit]
- British Columbia Ministry of Forests, Lands and Natural Resource Operations. Site Index Estimates by Site Series; British Columbia Ministry of Forests, Lands and Natural Resource Operations: Victoria, BC, Canada, 2013. Available online: https://www2.gov.bc.ca/assets/gov/environment/plants-animals-and-ecosystems/ecosystems/sibec-documents/sisubyregion2013.pdf (accessed on 12 May 2026).
- Fahlvik, N.; Agestam, E.; Eko, P.M.; Linden, M. Development of single-storied mixtures of Norway spruce and birch in Southern Sweden. Scand. J. For. Res. 2011, 26, 36–45. [Google Scholar] [CrossRef] [Scilit]
- Pretzsch, H.; Biber, P. Tree species mixing can increase maximum stand density. Can. J. For. Res. 2016, 46, 1179–1193. [Google Scholar] [CrossRef] [Scilit]
- Thrum, E.A.; Pretzsch, H. Growth–density relationship in mixed stands—Results from long-term experimental plots. For. Ecol. Manag. 2021, 483, 118909. [Google Scholar] [CrossRef] [Scilit]
- Martin, P.J. Design of regeneration standards to sustain boreal mixedwoods in western Canada. Int. For. Rev. 2005, 7, 135–146. [Google Scholar] [CrossRef] [Scilit]
- Martin, P.J.; Browne-Clayton, S.; Day, K.; Taylor, G. Improving regeneration performance standards: Comments based on early experience with three new approaches in British Columbia. In Thin Green Line Proceedings. A Symposium on the State-of-the-Art in Reforestation, Thunder Bay, ON; Colombo, S.J., Ed.; Ontario Forest Research Institute: Sault Ste Marie, ON, Canada, 2005; pp. 59–65. Available online: https://rngr.net/publications/tgl/improving-regeneration-performance-standards-comments-based-on-early-experience-with-three-new-approaches-in-british-columbia (accessed on 8 April 2026).
- Bergqvist, G. Wood volume yield and stand structure in Norway spruce understorey depending on birch shelterwood density. For. Ecol. Manag. 1999, 122, 221–229. [Google Scholar] [CrossRef] [Scilit]
- Jobidon, R. Density-dependent effects of northern hardwood competition on selected environmental resources and young white spruce (Picea glauca) plantation growth, mineral nutrition, and stand structural development ± a 5-year study. For. Ecol. Manag. 2000, 130, 77–97. [Google Scholar] [CrossRef] [Scilit]
- Larocque, G.R.; Marshall, P.L. Crown development in red pine stands. II. Relationships with stem growth. Can. J. For. Res. 1994, 24, 775–784. [Google Scholar] [CrossRef] [Scilit]
- Carr, S.; Larocque, G.R.; Luckai, N.; Bell, F.W. Effect of competition on individual white spruce production in young boreal mixedwood forests. Can. J. For. Res. 2020, 50, 726–735. [Google Scholar] [CrossRef] [Scilit]
- Larocque, G.R. Functional growth analysis of red pine trees under variable intensities of competition. For. Chron. 1998, 74, 728–735. [Google Scholar] [CrossRef] [Scilit]
- Larocque, G.R.; Marshall, P.L. Evaluating the impact of competition using relative growth rate in red pine (Pinus resinosa Ait.) stands. For. Ecol. Manag. 1993, 58, 65–83. [Google Scholar] [CrossRef] [Scilit]
- Burton, P.J. Some limitations inherent to static indices of plant competition. Can. J. For. Res. 1993, 23, 2141–2152. [Google Scholar] [CrossRef] [Scilit]
- Huuskonen, S.; Domisch, T.; Finér, L.; Hantula, J.; Hynynen, J.; Matala, J.; Miina, J.; Neuvonen, S.; Nevalainen, S.; Niemistö, P.; et al. What is the potential for replacing monocultures with mixed-species stands to enhance ecosystem services in boreal forests in Fennoscandia? For. Ecol. Manag. 2021, 479, 118558. [Google Scholar] [CrossRef] [Scilit]
- Ara, M.; Felton, A.M.; Holmstrom, E.; Petersson, L.; Berglund, M.; Johansson, U.; Nilsson, U. Pre-commercial thinning in Norway spruce-birch mixed stands can provide abundant forage for ungulates without losing volume production. For. Ecol. Manag. 2022, 520, 120364. [Google Scholar] [CrossRef] [Scilit]
- Béland, M.; Lussier, J.-M.; Bergeron, Y.; Longpré, M.-H.; Béland, M.I. Structure, spatial distribution and competition in mixed jack pine (Pinus banksiana) stands on clay soils of eastern Canada. Anal. For. Sci. 2003, 60, 609–617. [Google Scholar] [CrossRef] [Scilit]
- Stadt, K.J.; Huston, C.; Coates, K.D.; Feng, Z.; Dale, M.R.T.; Lieffers, V.J. Evaluation of competition and light estimation indices for predicting diameter growth in mature boreal mixed forests. Ann. For. Sci. 2007, 67, 477–490. [Google Scholar] [CrossRef] [Scilit]
- van Cleve, K.O.; Heal, W.; Roberts, D. Biomass of forest floor nitrogen supply for plant growth. Can. J. For. Res. 1986, 16, 1320–1326. [Google Scholar] [CrossRef] [Scilit]
- Maundrell, C.P. Effect of Aspen (Populus tremuloides (Michx.)) Overstory Removal on Productivity of an Aspen and White Spruce (Picea glauca (Moench) Voss) Mixedwood Stand. Master’s Thesis, University of Northern British Columbia, Prince George, BC, Canada, 2002. [Google Scholar] [CrossRef] [Scilit]
- Tham, A. Crop Plans and Yield Predictions for Norway Spruce (Picea abies (L.) Karst.) and Birch (Betula pendula Roth & Betula pubescens Ehrh.) Mixtures; Studia Forestalia Suecica; Swedish University of Agricultural Sciences (SLU): Uppsala, Sweden, 1994; Volume 195, pp. 1–21. [Google Scholar]
- Lieffers, V.J.; Pinno, D.B.; Stadt, K.J. Light dynamics and free-to-grow standards in aspen dominated mixedwood forests. For. Chron. 2002, 78, 137–145. [Google Scholar] [CrossRef] [Scilit]
- Simard, S.W.; Sachs, D.L.; Vyse, A.; Blevins, L.L. Paper birch competitive effects vary with conifer tree species and stand age in interior British Columbia forests: Implications for reforestation policy and practice. For. Ecol. Manag. 2004, 198, 55–74. [Google Scholar] [CrossRef] [Scilit]
- Armstrong, G.W. Considerations for boreal mixedwood silviculture: A view from the dismal science. For. Chron. 2014, 90, 44–49. [Google Scholar] [CrossRef] [Scilit]
- Parker, W.C.; Sharma, M. Influence of post-harvesting residual stand structure on canopy light transmittance in Ontario’s boreal mixedwood forests. For. Chron. 2018, 94, 35–46. [Google Scholar] [CrossRef] [Scilit]
- Knoke, T.; Ammer, C.; Stimm, B.; Mosandl, R. Admixing broadleaved to coniferous tree species: A review on yield, ecological stability and economics. Eur. J. For. Res. 2008, 127, 89–101. [Google Scholar] [CrossRef] [Scilit]
- Kayahara, G.J. First Nation Herbicide. The (Ontario) Professional Forester. Number 229: 7–9. 2018. Available online: https://opfa.ca/wp-content/uploads/2018/04/OPFA-Newsletter_march2018.pdf (accessed on 28 April 2026).
- Légaré, S.; Paré, D.; Bergeron, Y. The responses of black spruce growth to an increased proportion of aspen in mixed stands. Can. J. For. Res. 2004, 34, 405–416. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.