


Abstract
There has been considerable urban development in the Darwin region over the last twenty years; as for most fauna in Australia since colonisation, the potential effects to the bird assemblage were expected to be disastrous. To provide a broad overview of changes, bird survey data from 1998 and 2018 were extracted from BirdLife Australia’s ‘Atlas of Australian Birds’ database. A total of 165 species were categorised into primary food source feeding guilds and levels of food specialisation. This was integrated into ArcGIS along with land use change mapping from 1998 and 2018 to investigate its impact on bird assemblages. There was no significant change in overall species numbers when all sites were analysed. However, when sites were separated into those with increased urbanisation or decreased greenspace, several sites showed a significant change in the number of species. For the majority of species, analysis of primary food types found no difference in the proportion of species within the assemblages between 1998 and 2018, regardless of the level of urbanisation or greenspace; the exception being those species that primarily feed on insects, where the difference was just significant. An analysis using bird community data sorted into levels of food specialisation also found no difference between 1998 and 2018 despite habitat changes. These findings suggest that although there has been considerable urban development in the Darwin region, bird communities are remaining relatively stable.
1. Introduction
Global population trends show that humans are moving from rural areas into cities at a considerable rate, and once sparsely populated regions are being transformed to cope with the influx of people [1,2]. Subsequently, urbanisation is now widely considered a major threat to biodiversity conservation [3,4,5].
Species’ responses to urbanisation can vary significantly [6]; however, prior to the 1990s, very few ecological studies were undertaken in urban areas due to them being considered unviable habitats for faunal populations and, ergo, immaterial from a conservation standpoint [7]. It is now shown that urban areas support an array of species that have been able to tolerate or adapt to the highly fragmented new environments but, due to a lack of appropriate knowledge, the success of urban conservation programmes may be hampered [4]. There is little doubt that avian assemblages are greatly altered by urbanisation; many bird species unable to adapt to the suddenly changed environment will often move out of an area resulting in diminished biodiversity and allowing invasive species to move in [4,8,9]. Other species can benefit from urbanisation; these are often birds with a more generalist diet and life-history traits that are conducive to living in a fragmented habitat [10].
Whilst studies of bird populations in urban areas abound in the temperate zones of both the Northern and Southern hemispheres, research into tropical urban avian communities is scant [11]. This trend is continued in Australian studies with the majority of research being undertaken in the temperate regions, predominantly in the two heavily populated states of New South Wales and Victoria. In contrast, this study is situated in the monsoonal tropics of northern Australia; specifically, in Darwin, the capital of the Northern Territory (NT). There has been targeted research on a range of species and thorough overviews of bird distributions within the region [12,13,14], with more detailed studies of shorebirds [15,16,17,18] and mangrove assemblages [19,20,21]. To date, however, there have been no studies of trends in terrestrial bird assemblages as the city has grown. Given the increased rate of urbanisation in the global tropics [22], coupled with high levels of biodiversity in the zone [11,23,24,25], there is an increasing need to gather data to better understand how bird communities are coping with the rising encroachment of human habitation. This is particularly interesting in Darwin as, unlike all other urban centres in Australia, Darwin has no introduced birds, so all the adaptation is being undertaken by native species as their environment is changed.
In the nearly 45 years since Darwin was severely damaged by Cyclone Tracy, where 70–80% of dwellings were destroyed [26,27], the city has grown from a perceived ‘frontier town’ to be a modern capital city. This development has seen an increase of over 20 new suburbs in the greater Darwin area and surrounds, and land once considered bush or rural properties is now being subdivided into urban blocks. One of the most common effects of urbanisation is the increasing prevalence of exotic species [28,29,30]; however, this has not occurred in the Darwin region with only four species listed as ‘foreign invaders’, none of which have established permanent breeding populations [31].
In this paper, we shall test this theory by investigating the response of the terrestrial avian assemblages in the Darwin region to urban expansion and land use change over the past 20 years.
2. Materials and Methods
2.1. Study Area
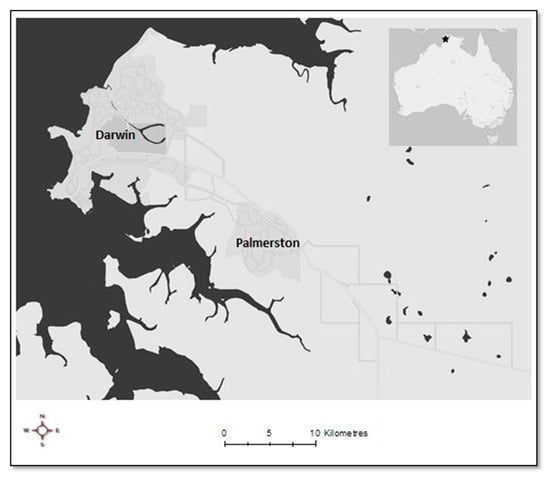
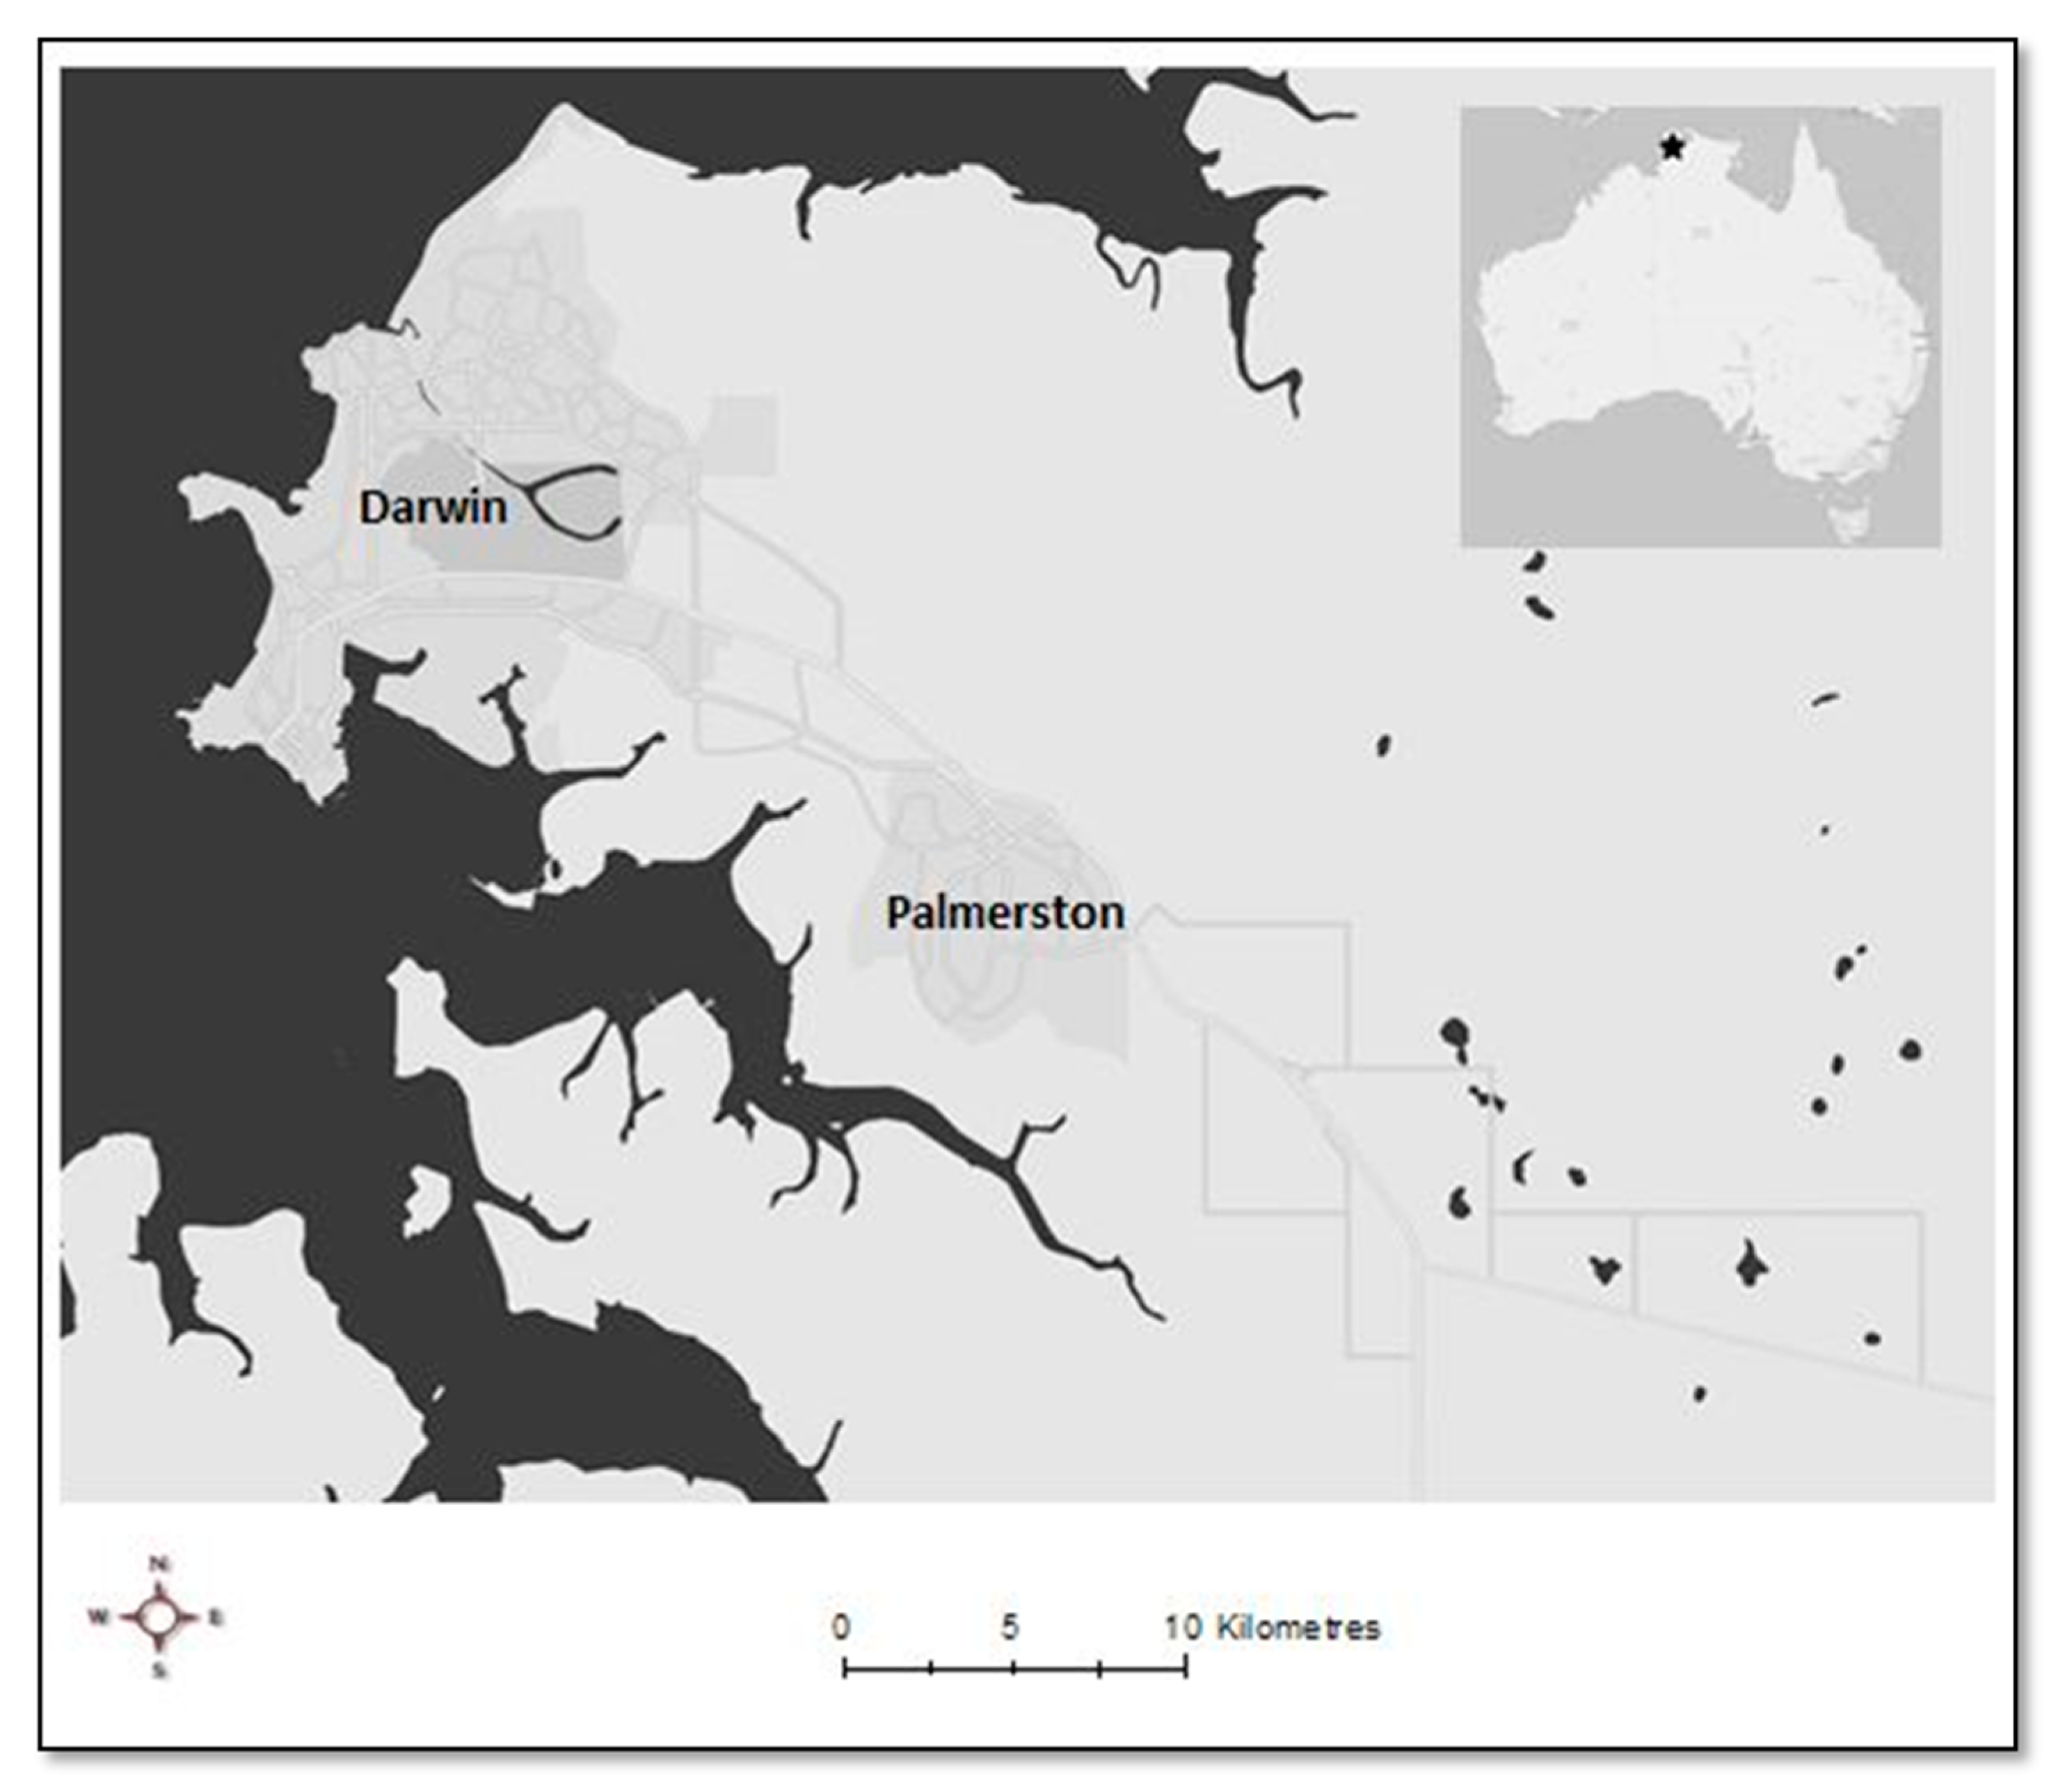
Darwin (12.4634° S, 130.8456° E) is situated on the north coast of Australia, a landscape dominated by tropical savanna (Figure 1).
Figure 1.
Study area of the Greater Darwin region (map data sources: Esri, DeLorme, HERE, USGS, Intermap, iPC, NRCAN, Esri Japan, METI, Esri China (Hong Kong), Esri (Thailand), MapmyIndia, Tomtom).
The population of approximately 140,000 [32] constitutes an increase of nearly 60,000 people in twenty years [33]. The climate is monsoonal and experiences distinct annual dry (May to September) and wet (November to April) seasons with transitional periods in between. Mean annual rainfall is approximately 1700 mm; the mean minimum and maximum temperatures range from 19.3° to 25.3° and 30.6° to 33.3°, respectively [34]. Compared to other major Australian capital cities, housing density is low; under 20 private dwellings per square kilometre as opposed to between 150 to 200 per square kilometre in Sydney and Melbourne [35]. A combination of urban and periurban environments in the Darwin region provides resources for avian populations that are typically unavailable outside of this area in the dry season.
2.2. Spatial Data
To investigate broad-scale changes in urbanisation, Landsat satellite imagery of the study area from April 1998 and 2018 was obtained from the United States Geological Survey’s Global Visualization Viewer (GloVis), with 1998 imagery obtained from the Landsat 4 and 5 Thematic Mapper (TM) satellite and 2018 imagery taken by the Landsat 8 Operational Land Imager (OLI) and Thermal Infrared Sensor (TIRS) (Table A1 and Table A2). April marks the end of the wet season in Darwin, allowing for images with minimal cloud cover and maximum vegetation growth. Images were clipped in ArcGIS version 10.4.1 [36] to a shapefile of Darwin region localities provided by the Northern Territory Government Department of Environment and Natural Resources and then imported into SAGA GIS version 7.3.0 [37]. Classification of land use types was carried out via geographic object-based image analysis (GEOBIA). In traditional pixel-based image classification, classes are assigned per pixel; however, GEOBIA uses segmentation and classification to better replicate what the human eye perceives [38,39]. The segmentation process combines pixels of similar spectral properties into objects in the form of polygons, and these can then be classified using either supervised or unsupervised techniques [40]. After automated segmentation in SAGA GIS, the two clipped images were classified by assigning ‘training sites’ (essentially selecting a minimum number of polygons and ascribing them a land use type) and then running a supervised classification. The resulting vector layers were then manually edited using the original satellite image to reassign any misclassified polygons. The initial uncorrected GEOBIA and user-corrected images were then re-imported back into ArcGIS, where fifty accuracy assessment points were randomly generated and an error matrix was constructed to assess both the producer (SAGA) and user (human) accuracy when assigning classification. For all map classifications satellite imagery, aerial photographs and Google Earth Pro version 7.3.2.5776 (64 bit) were used to assist in the accuracy assessment; however, due to the retrospective nature of the earlier imagery, only the 2018 images could be further checked, if required, using ground control points.
2.3. Bird Survey Data
Survey data were extracted from the BirdLife Australia ‘Atlas of Australian Birds’ database (hereafter referred to as the ‘Bird Atlas’) for the years 1998 and 2018. Several types of surveys compiled these data: systematic bird surveys of 2 ha, 5 km and 500 m; unstandardised bird surveys, either along a fixed route or incidental; bird list surveys and the Shorebird 2020 surveys (a record of shorebird sightings not necessarily in coastal habitats). All records include a location, latitude and longitude, dates and species common names. In most records, a time is recorded and whether there is any breeding activity. Sighting notes of interest are sometimes included.
As the focus of the project was on terrestrial, predominantly diurnal species, Bird Atlas records were excluded if the species was almost exclusively nocturnal, was a waterbird or seabird (except Magpie Geese, Anseranas semipalmata), or the species was considered ‘vagrant’. Using information from BirdLife Australia [41], the Atlas of Living Australia [42] and Australian Bird Data Version 1.0 [43], the feeding preferences of species were categorised from most preferred to occasional.
To give a general overview of any assemblage changes, the records of 1998 and 2018 were categorised into the following primary food sources: fruit, insects, invertebrates, nectar, omnivore, raptor, scavenger, seed, vegetation or vertebrate. If a species was considered to feed on two types of food source equally, both were considered the primary food source. Species were sorted by their level of specialisation: whether they had one, two, three or more food sources (Table A3).
2.4. Integration of Data
Following Hahs and McDonnell [44] and Conole and Kirkpatrick [30], the final edited spatial images were re-imported into ArcGIS and a 1 × 1 km grid was overlaid. The modified Bird Atlas data from 1998 and 2018 were then added as point layer files. As with Conole and Kirkpatrick [30], the locations were taken from the coordinates provided. The grid cells that contained records from both 1998 and 2018 were extracted for each year, and the level of land use type in each grid cell was calculated. Land use types were combined and simplified into greenspace (woodland, grass and forest), coastal (mangrove, sea and sand), urbanised (suburban, periurban, building and road), water and bare earth. Percentage change of greenspace and urbanisation between 1998 and 2018 was calculated for the relevant grid cells.
2.5. Statistical Analysis
Data were analysed using R version 3.6.1 [45].
Analysis of variance (ANOVA) was used to investigate whether the site and year had an effect on overall species numbers; paired t-tests were then used to examine the significance of any changes between 1998 and 2018 in those sites where urbanisation had increased or greenspace had decreased. The analysis was repeated to assess species’ primary food source categories.
Finally, effects of land change on feeding specialisation numbers in bird assemblages were also explored. To do this, assemblage species proportions of one, two, three or more food sources were analysed for grid cells that were determined to have had an increase in urbanisation, a decrease in urbanisation, no change in the amount of urbanisation, an increase in greenspace or a decrease in greenspace.
3. Results
3.1. Spatial Data
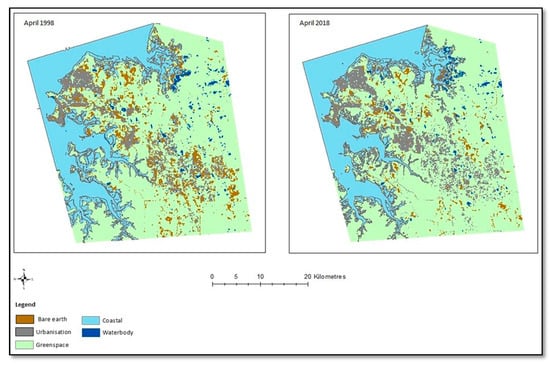
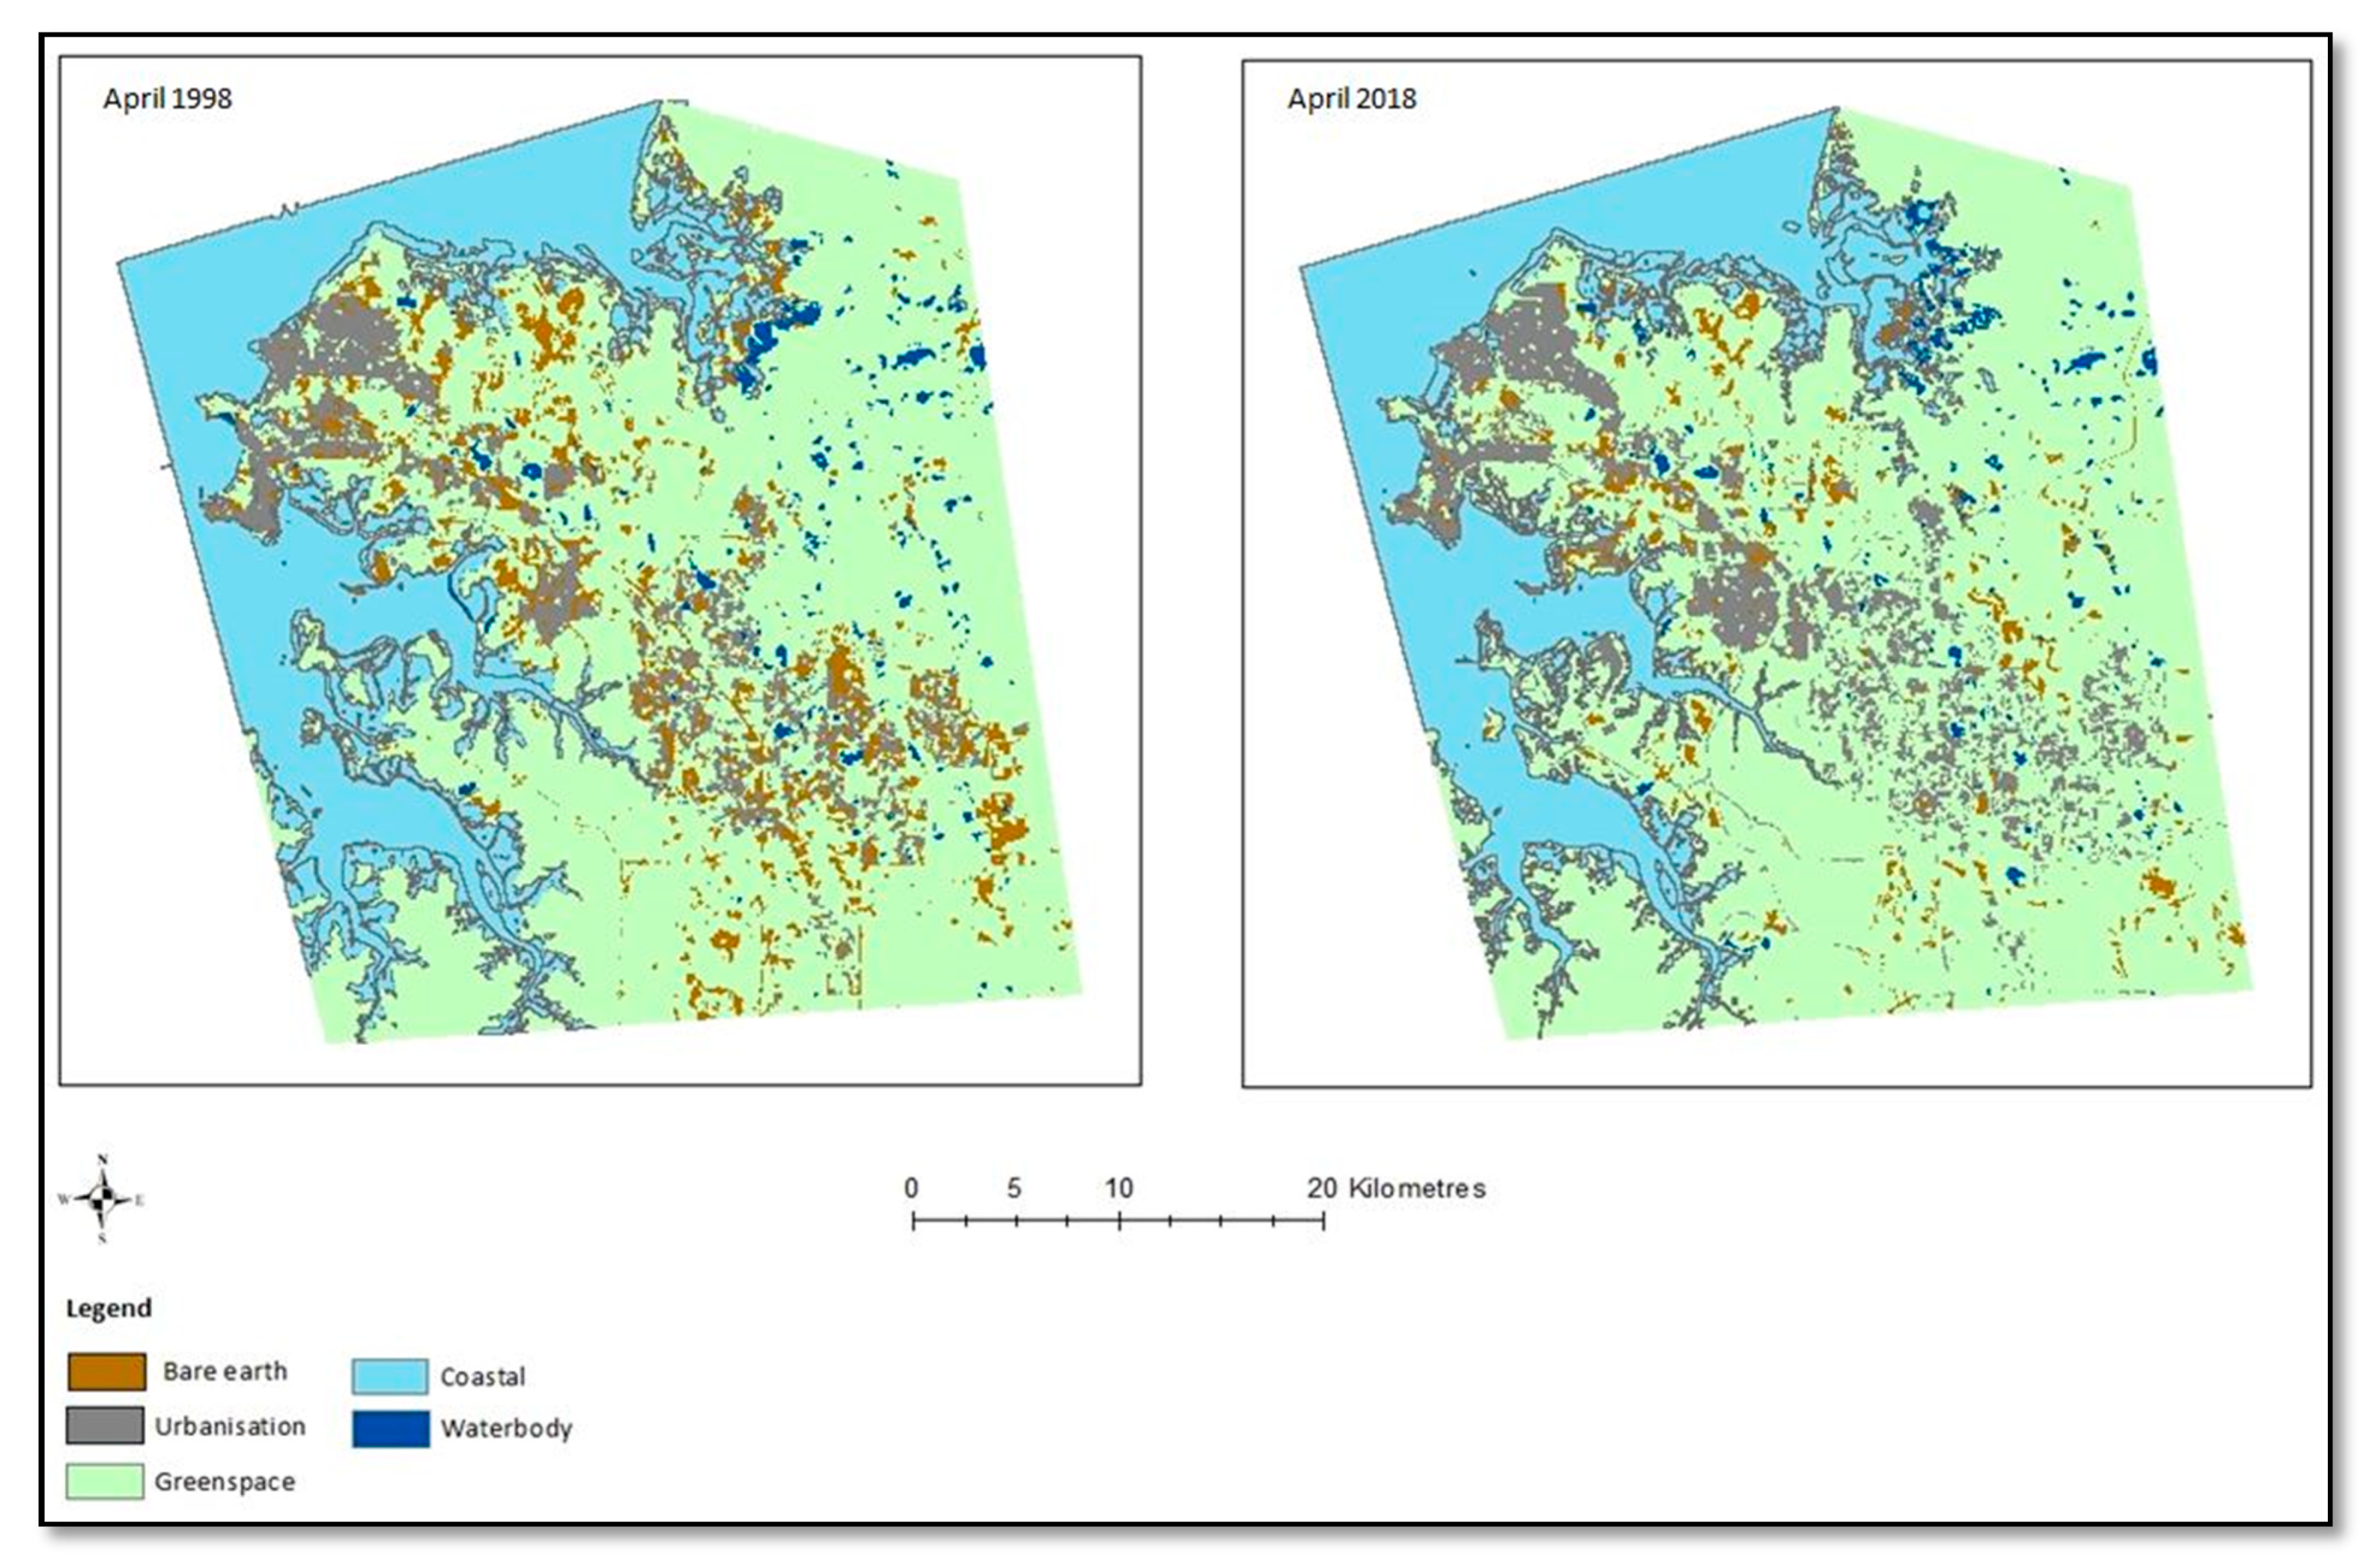
Results of the GEOBIA found that urbanised areas increased from 114 to 151 km2, a percentage increase of almost 3% of the total land mass measured. Greenspace, too, increased by just under 5%; 986 to 1045 km2.
For the 1998 imagery, overall accuracy was 75% (producer accuracy 72%; user accuracy 84%). The 2018 imagery returned an overall accuracy of 87% (84% producer and 90% user accuracies). This difference in accuracy was expected due to the quality differences in the Landsat 5 versus Landsat 8 imagery. Final corrections were made to the classified imagery before extraction of the relevant land use data for analysis (Figure 2).
Figure 2.
Final classified images of land use change with combined land classes.
3.2. Bird Atlas Data
Overall, there were 23 grid cells that contained Bird Atlas records from both 1998 and 2018. Of these, nine showed an increase in urbanisation ranging from 0.9 to 58.2%; eight indicated a decrease in urbanisation and six were recorded as no change. A decrease in greenspace was found in 15 grid cells, and 8 were determined to have had an increase. No species considered primarily a scavenger was found in the 23 grid cells.
3.3. Overall Change in Species Numbers
In total, 165 individual species were represented in the bird records used. Of these, 23 species were recorded in 1998 only and 19 in 2018 only (Table A4). All sites showed a change in species numbers between 1998 and 2018; however, when all sites were included, there was no significant change in total species numbers (F = 1.1909, p = 0.3999 and F = 1.9395, p = 0.1707, respectively).
Focussing on those sites where urbanisation had increased or greenspace had decreased over the 20-year period, changes in species numbers were more distinctive. Although sites are listed numerically, this is for brevity, and they are not necessarily the same location.
Where urbanisation had increased, of the nine sites analysed, five sites showed an increase in overall species numbers with four of these increases found to be statistically significant (p < 0.05). Examination of sites where species numbers decreased found two where the decrease was significant and two where there was no statistical significance (Table 1).
Table 1.
Results of paired t-test for difference in the overall number of bird species per site between 1998 and 2018 in areas where urbanisation has increased (df = 8).
In sites where there was a decrease in greenspace, the majority (10 out of 15) displayed an increase in species numbers, but of these, only three were found to be significant. The remaining five sites where a decrease in species was recorded again found three with statistical significance (Table 2).
Table 2.
Results of paired t-test for difference in the overall number of bird species per site between 1998 and 2018 in areas where greenspace has decreased (df = 14).
3.4. Changes to Species Numbers with Regard to Primary Food Sources
Species for each site were categorised by their primary food source, and changes in numbers initially were record as either an increase, decrease or no change for each food source.
In areas where urbanisation had increased, site 6 (increase in urbanisation of 5.8%) showed an increase in every species type, whereas site 4, which had the highest increase in urbanisation of any site (58.2%), displayed a decrease in almost every species type bar one, in which there was no change (Table 3).
Table 3.
Change in species numbers across sites where urbanisation has increased; I = increase, D = decrease and NC = no change.
Subsequent analysis found that there was no significant change in species numbers by primary food source overall (Table 4).
Table 4.
Change in species numbers across sites where greenspace has decreased; I = increase, D = decrease and NC = no change.
When investigating those sites where greenspace had decreased, one site (7) showed an increase in every species type despite having a greater reduction in greenspace (14.2%) than either site 6 (13.4%) or site 8 (5.3%), both of which showed a reduction in every species type except those that feed primarily on vegetation (Table 4).
Unlike those sites where urbanisation had increased, analysis of changes in species numbers in the sites where greenspace had decreased found a significant change in those species whose primary food source was insects (p < 0.05). Some change was noted for raptors too, but this was not quite statistically significant (p = 0.06) (Table 5).
Table 5.
Results of paired t-test for difference in the number of bird species by primary food source between 1998 and 2018 in areas where greenspace has decreased (df = 14).
3.5. Changes to Bird Assemblages with Regard to Primary Food Sources
Alongside changes to the number of species within bird communities over time, it was also pertinent to investigate whether the proportion of feeding guild types was altered within assemblages due to changing habitats, specifically in those sites where urbanisation increased or greenspace decreased.
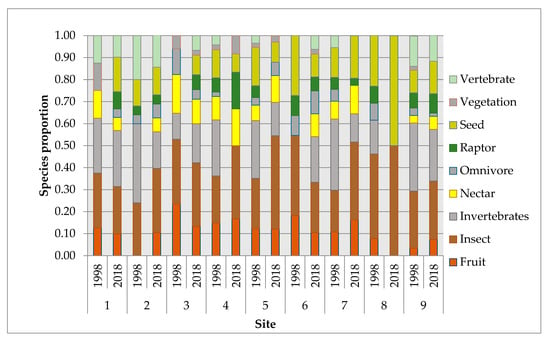
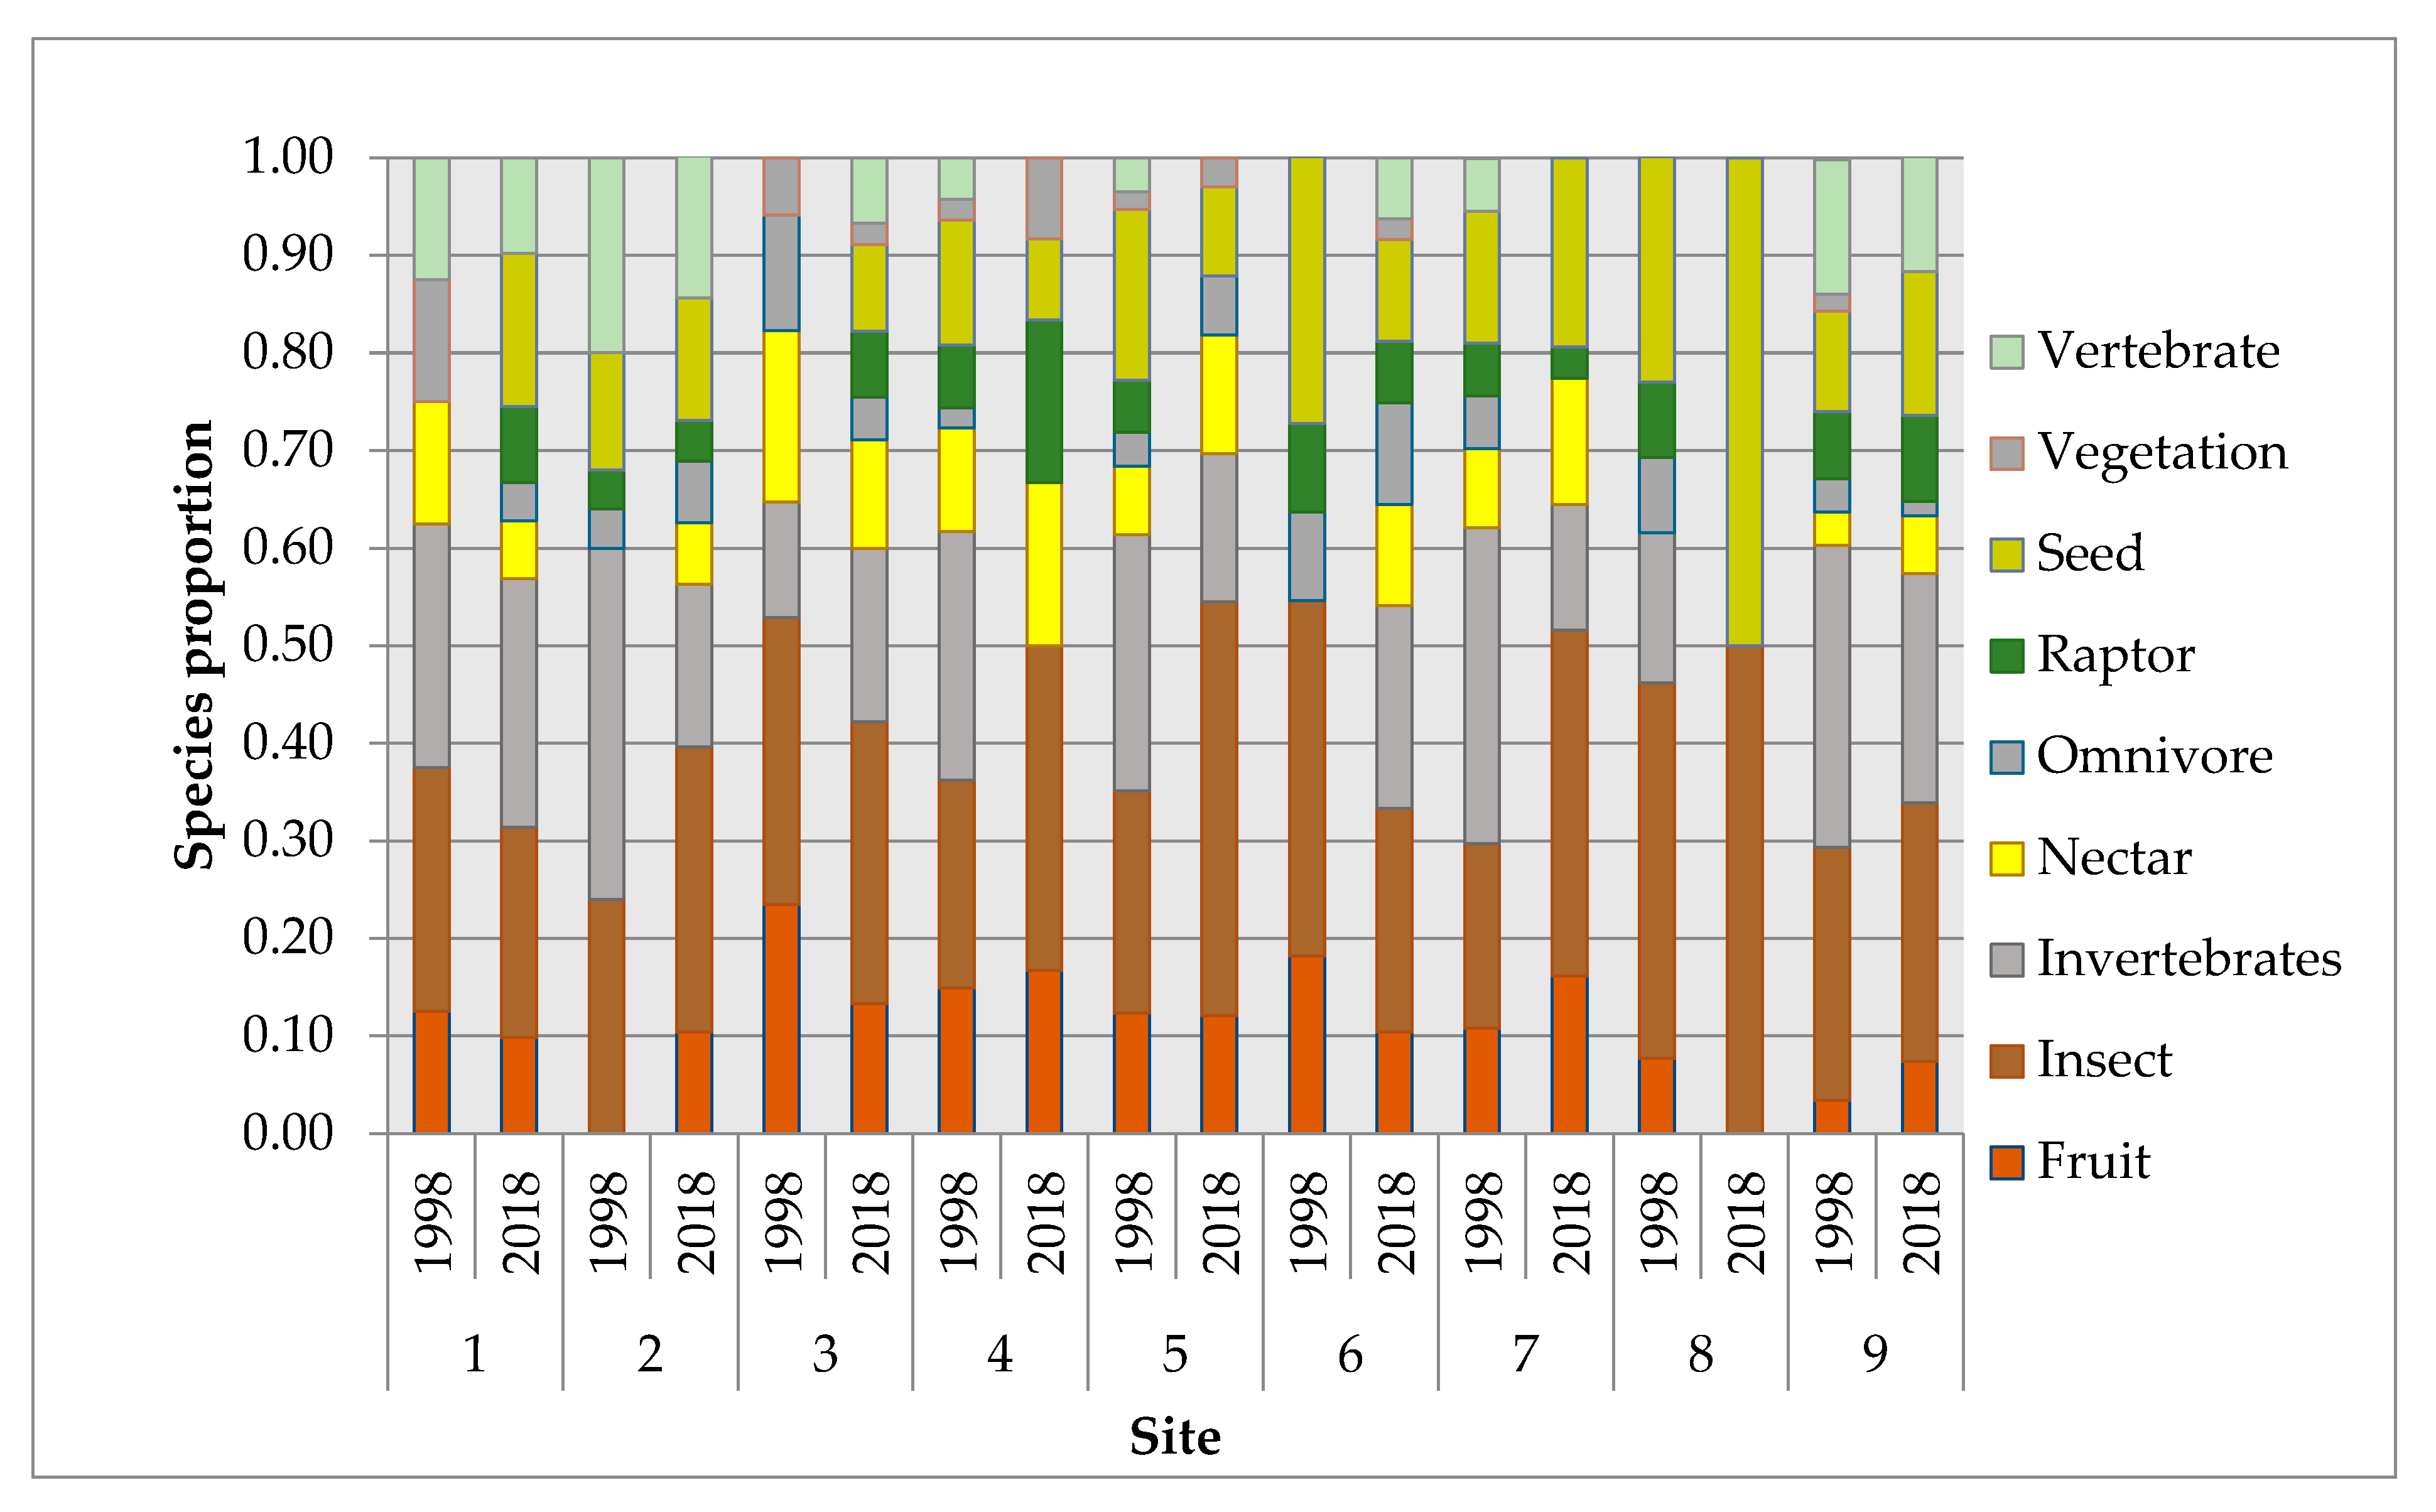
A comparison of the proportions of species type for each site where urbanisation was found to have increased is shown in Figure 3.
Figure 3.
Proportion of species by primary food source at sites where urbanisation has increased.
Subsequent analysis showed an increase in urbanisation resulted in no significant difference in the proportion of species of different primary food sources between 1998 and 2018.
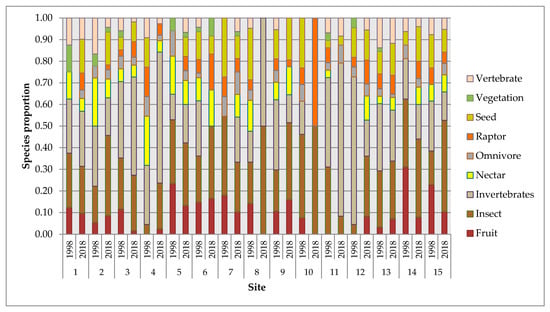
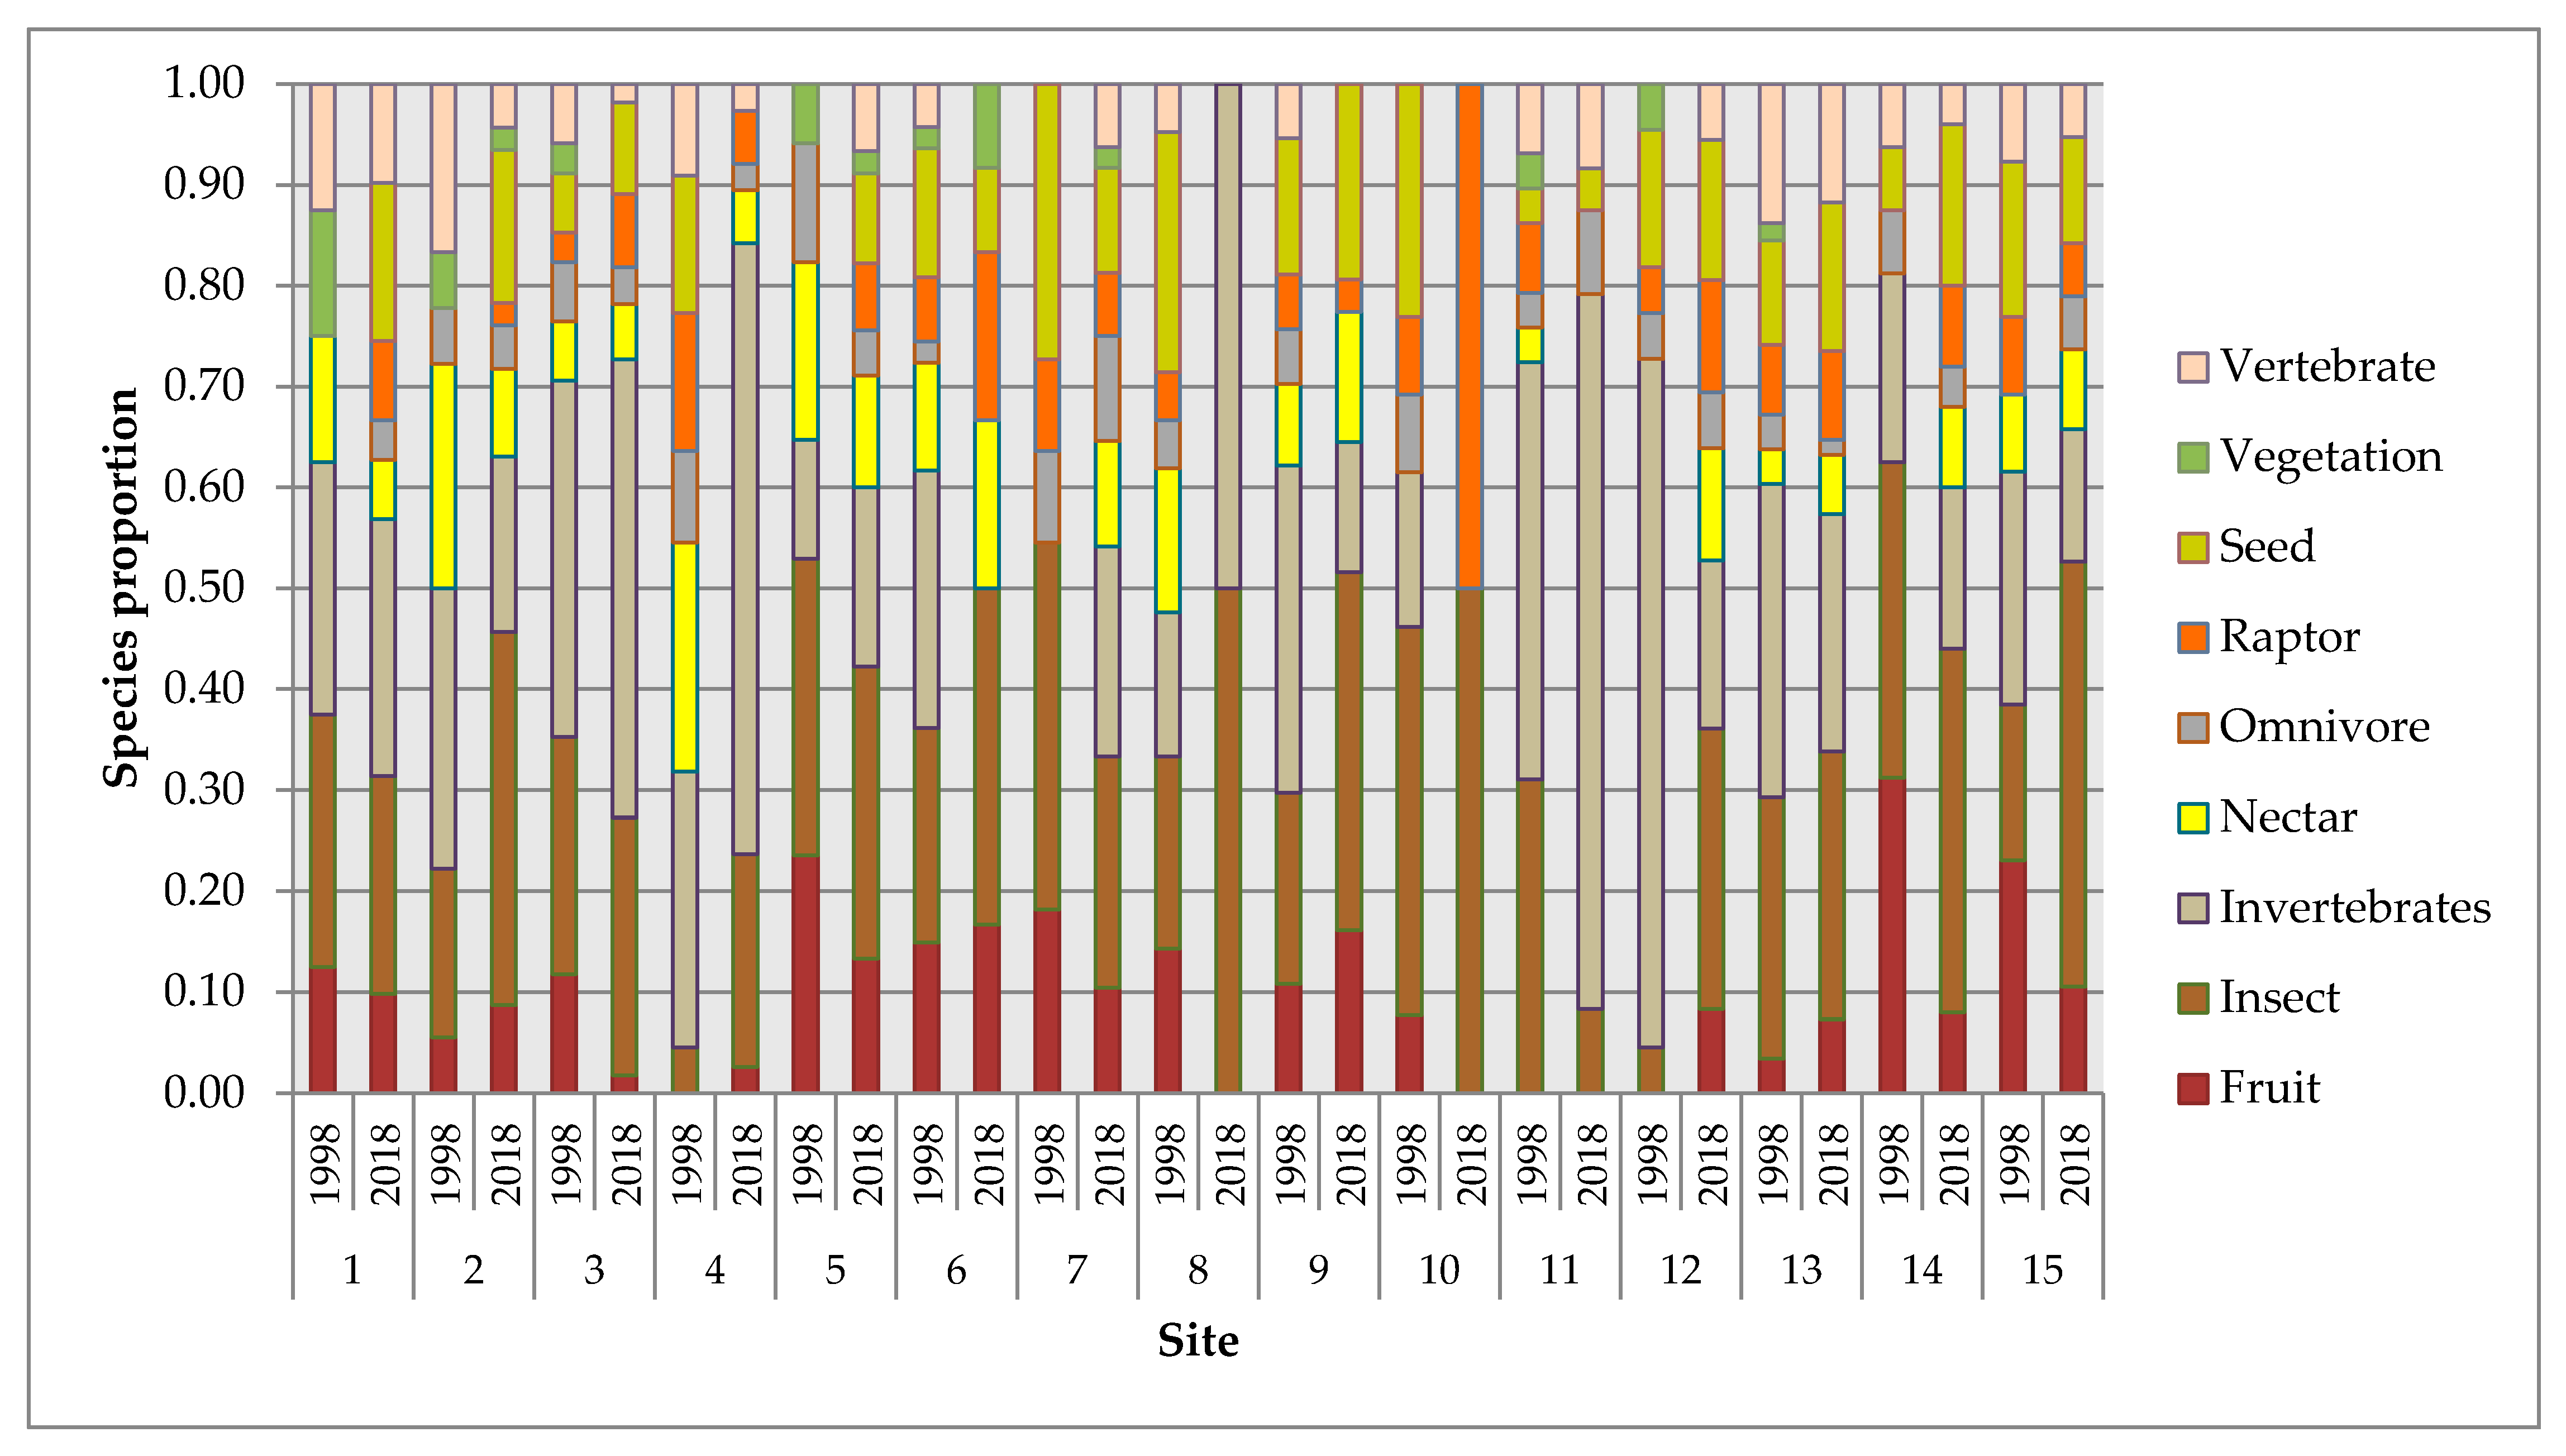
However, in grid cells that had a decreased amount of greenspace, a slight significant difference was shown in those species that chiefly feed on insects, and there is a suggestion of change in those species that primarily feed on fruit, although this was not found to be significant (Table 6).
Table 6.
Results of paired t-test for difference in the proportion of bird species by primary food source between 1998 and 2018 in areas where greenspace has decreased (df = 14).
A comparison of species proportion by primary food source for those grid cell sites where greenspace had decreased over the 20-year period is shown in Figure 4.
Figure 4.
Proportion of species by primary food source at sites where greenspace has decreased.
3.6. Levels of Specialisation
The levels of feeding specialisation within bird communities between 1998 and 2018 showed no significant change despite varying levels of urbanisation and greenspace (Table 7).
Table 7.
Results of paired t-test for difference in the proportion of feeding specialisation in bird assemblages with changing land use.
4. Discussion
Of the 258 birds species recorded in the Darwin area (escaped or introduced species and vagrants excluded), approximately 40% are considered resident [46] with the remaining species described as mobile. It has previously been thought that mobile species cope better with urbanisation than sedentary species [47,48], although other studies have suggested that highly mobile species may be more vulnerable to habitat changes due to their dependence on larger habitat patches and generally far-reaching home ranges [49,50,51]. Furthermore, there is also evidence to suggest that the fragmentation of habitats caused by urbanisation is going some way to changing the status of some birds from ‘visitor’ to ‘resident’ [52,53,54].
That there is a significant difference, albeit slight, in the proportion of those species that primarily feed on insects in areas where greenspace has decreased may possibly be attributed to the establishment of urban gardens. Although the size of the greenspace has decreased overall in these locations, in 73% of the grid cells analysed, the proportion of species that preferred insects increased; in contrast, only 47% of grid cells contained an increase in fructivores. It may be that the plants in these gardens attract a larger array of insects, thus providing more appealing spaces for insectivores. Numerous studies have indicated that the bird species that tend to thrive in urban environments are those that nest in cavities or canopies (sites less likely to be disturbed by human activity) and are more likely to be granivorous or omnivorous, whereas those species that avoid urban areas are those that predominantly nest in shrubs or trees or at ground level and have a more specialised diet, frequently insectivores [29,30,55]. However, these characteristics have been determined from research undertaken in either the Northern Hemisphere or the temperate zones of the Southern Hemisphere, places where garden vegetation is often vastly different to that of the original habitat. Suburban gardens of the Darwin region often contain native plant species alongside exotics, and this mixture may be enough to maintain, or even increase, insect numbers.
That there is no significant difference in the levels of feeding specialisation in bird assemblages is something of a surprise, as it would be fair to assume that more generalised species would be increasing and those species with one preferred food source would be forced out, particularly in areas of urban increase. Homogenisation of habitat is an oft-quoted result of urbanisation [5,56,57], but from this broad overview, it appears not to be affecting the composition of bird communities in the Darwin region. Further research into the characteristics of species making up urban assemblages will go some way to better understanding why this may be.
Invasion by feral species is a frequent result of an increased human presence in an area [29,30,58]. Many bird species that are unable to adapt to the suddenly changed environment will often move out of an area resulting in diminished biodiversity and allowing invasive species to move in [4,8,9]. Other species can benefit from urbanisation; these are often birds with a more generalist diet and life-history traits that are conducive to living in a fragmented habitat [10].
The only feral species in the records was Columba livia—the common pigeon, rock dove or rock pigeon. This species was recorded in the 1998 records only, most likely due to an eradication programme undertaken by the Parks and Wildlife Commission, NT, beginning in 1996, that saw the species considered eradicated from the Darwin area by 2004 [59,60]. The lack of established feral bird populations in the Darwin region could, potentially, suggest that native bird species are filling the ‘urban exploiter’ or ‘suburban adapter’ niche that is commonly filled by exotic species in other cities, but there is little or no research to show what these species may be. Additionally, a unique aspect of the Darwin region is that it is the only capital in Australia where urban fires are a regular annual occurrence. The city is located within the monsoonal tropics; a landscape dominated by tropical savannas, experiencing frequent fires during the prolonged dry season from May to October, often within just metres of suburban housing areas [61]. In addition to wildfires, many of these fires are prescribed, being undertaken by various land-management bodies as part of a yearly landscape management approach [62,63]. Whether these annual fires are in some way supporting and maintaining the local bird assemblages whilst preventing invasive species from establishing populations is an intriguing question. Research into the combined impact of urban fires and human modification of the environment on local bird populations over time is ongoing; it is hoped that the results will go some way towards answering this question.
5. Conclusions
Whilst very transient, the population of Darwin and its surrounds has grown significantly between the years 1998 and 2018, and urbanisation has expanded more than 50 km from the city centre. Despite this, this general overview of bird assemblages shows that although species numbers fluctuate, avian communities appear to be stable. The increase in the insectivorous species may be due to the establishment, maturity and vegetative composition of suburban gardens. This may potentially signify a shift in the species diversity of the area; however, further research is needed to investigate this.
Author Contributions
S.E.F. conceived, designed and performed the experiments. S.E.F. analysed the data. S.E.F. and A.C.E. wrote the paper. P.W., S.T.G. and T.G.W. provided guidance and comments on the manuscript. All authors have read and agreed to the published version of the manuscript.
Funding
This study is part of a larger Ph.D. project that is supported by Charles Darwin University and the Australian Government via the Research Training Programme scholarship.
Institutional Review Board Statement
Not applicable.
Data Availability Statement
The authors confirm that the data supporting the findings of this study are available within the article, its Appendices, and Australian Bird Data Version 1.0 (https://doi.org/10.6084/m9.figshare.1499292_D8, access date 10 September 2019) at http://www.birdsaustralia.com.au/ (access date 19 June 2019) and https://www.ala.org.au/ (access date 1 September 2019).
Acknowledgments
The authors would like to thank Andrew Silcox and BirdLife Australia for access to bird data records.
Conflicts of Interest
The authors declare no conflict of interest.
Appendix A. Landsat Satellite Specifications
Table A1.
Landsat 4 and Landsat 5 Thematic Mapper (TM) 1998 imagery (Data Taken from USGS [64,65]).
Table A2.
Landsat 8 and 9 Operational Land Imager (OLI) and Thermal Infrared Sensor (TIRS) 2018 imagery (Data Taken from USGS [64,65]).
Appendix B. Bird Species
Table A3.
Total bird species recorded.
Table A4.
Bird species recorded in 1998 only or 2018 only.
References
- Zhang, X.Q. The trends, promises and challenges of urbanisation in the world. Habitat. Int. 2016, 54, 241–252. [Google Scholar] [CrossRef] [Scilit]
- Fund, U.N.P. World Population Trends. 2017. Available online: https://www.unfpa.org/world-population-trends (accessed on 2 March 2019).
- Sewell, S.R.; Catterall, C.P. Bushland modification and styles of urban development: Their effects on birds in south-east Queensland. Wildl. Res. 1998, 25, 41–63. [Google Scholar] [CrossRef] [Scilit]
- Cleary, G.P.; Parsons, H.; Davis, A.; Coleman, B.R.; Jones, D.; Miller, K.; Weston, M.A. Avian Assemblages at Bird Baths: A Comparison of Urban and Rural Bird Baths in Australia. PLoS ONE 2016, 11, e0150899. [Google Scholar] [CrossRef] [Scilit]
- Bellocq, M.I.; Leveau, L.M.; Filloy, J. Urbanization and Bird Communities: Spatial and Temporal Patterns Emerging from Southern South America. In Ecology and Conservation of Birds in Urban Environments; Springer Science and Business Media LLC: New York, NY, USA, 2017; pp. 35–54. [Google Scholar]
- Evans, K.L.; Chamberlain, D.; Hatchwell, B.J.; Gregory, R.; Gaston, K.J. What makes an urban bird? Glob. Chang. Biol. 2010, 17, 32–44. [Google Scholar] [CrossRef] [Scilit]
- Garden, J.; McAlpine, C.; Peterson, A.; Jones, D.; Possingham, H. Review of the ecology of Australian urban fauna: A focus on spatially explicit processes. Austral Ecol. 2006, 31, 126–148. [Google Scholar] [CrossRef] [Scilit]
- Lancaster, R.K.; Rees, W.E. Bird communities and the structure of urban habitats. Can. J. Zool. 1979, 57, 2358–2368. [Google Scholar] [CrossRef] [Scilit]
- Bezzel, E. Birdlife in intensively used rural and urban environments. Ornis Fennica 1985, 62, 90–95. [Google Scholar]
- Blair, R.B. Birds and Butterflies Along Urban Gradients in Two Ecoregions of the United States: Is Urbanization Creating a Homogeneous Fauna? In Biotic Homogenization; Lockwood, J.L., McKinney, M.L., Eds.; Springer US: Boston, MA, USA, 2001; pp. 33–56. [Google Scholar]
- Wolff, P.J.; DeGregorio, B.A.; Rodriguez-Cruz, V.; Mulero-Oliveras, E.; Sperry, J.H. Bird Community Assemblage and Distribution in a Tropical, Urban Ecosystem of Puerto Rico. Trop. Conserv. Sci. 2018, 11, 1940082918754777. [Google Scholar] [CrossRef] [Scilit]
- Noske, R.A. The status and ecology of the white-throated grasswren Amytornis woodwardi. Emu 1992, 92, 39–51. [Google Scholar] [CrossRef] [Scilit]
- Noske, R.A. Breeding biology, demography and success of the rufous-banded honeyeater, Conopophila albogularis, in Darwin, a monsoonal tropical city. Wildl. Res. 1998, 25, 339–356. [Google Scholar] [CrossRef] [Scilit]
- Franklin, D.C.; Whitehead, P.J.; Pardon, G.; Matthews, J.; McMahon, P.; McIntyre, D. Geographic patterns and correlates of the decline of granivorous birds in northern Australia. Wildl. Res. 2005, 32, 399–408. [Google Scholar] [CrossRef] [Scilit]
- Crawford, D.N. Birds of Darwin Area, with Some Records from Other Parts of Northern Territory. Emu Austral Ornithol. 1972, 72, 131–148. [Google Scholar] [CrossRef] [Scilit]
- Crawford, D. Waterbirds: Indices and Fluctuations in Dry-Season Refuge Areas, Northern Territory. Wildl. Res. 1979, 6, 97–103. [Google Scholar] [CrossRef] [Scilit]
- Lilleyman, A.; Hensen, B.J. The occurrence of the Asian subspecies of the Gull-billed Tern (‘Gelochelidon nilotica affinis’) in the Darwin region, Northern Territory. North. Territ. Nat. 2014, 25, 12–17. [Google Scholar]
- Lilleyman, A.; Franklin, D.C.; Szabo, J.K.; Lawes, M. Behavioural responses of migratory shorebirds to disturbance at a high-tide roost. Emu Austral Ornithol. 2016, 116, 111–118. [Google Scholar] [CrossRef] [Scilit]
- Noske, R.A. The breeding biology of the Mangrove Gerygone, Gerygone laevigaster, in the Darwin region, with notes on brood parasitism by the Little Bronze-cuckoo, Chrysococcyx minutillus. Emu Austral Ornithol. 2001, 101, 129–135. [Google Scholar] [CrossRef] [Scilit]
- Mohd-Azlan, J.; Noske, R.A.; Lawes, M. Avian species-assemblage structure and indicator bird species of mangroves in the Australian monsoon tropics. Emu Austral Ornithol. 2012, 112, 287–297. [Google Scholar] [CrossRef] [Scilit]
- Mohd-Azlan, J.; Noske, R.A.; Lawes, M.J. The Role of Habitat Heterogeneity in Structuring Mangrove Bird Assemblages. Divers 2015, 7, 118–136. [Google Scholar] [CrossRef] [Scilit]
- Population Division of the United Nations Department of Economic and Social Affairs. 2018 Revision of World Urbanization Prospects; United Nations: New York, NY, USA, 2018. [Google Scholar]
- Ridpath, M.G. Ecology in the wet-dry tropics: How different? Proc. Ecol. Soc. Aust. 1985, 13, 3–20. [Google Scholar]
- Mittermeier, R.A.; Myers, N.; Thomsen, J.B.; Da Fonseca, G.A.B.; Olivieri, S. Biodiversity Hotspots and Major Tropical Wilderness Areas: Approaches to Setting Conservation Priorities. Conserv. Biol. 1998, 12, 516–520. [Google Scholar] [CrossRef] [Scilit]
- Gaston, K.J. Global patterns in biodiversity. Nat. Cell Biol. 2000, 405, 220–227. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bureau of Meteorology. Severe Tropical Cyclone Tracy. 2020. Available online: http://www.bom.gov.au/cyclone/history/tracy.shtml (accessed on 13 January 2020).
- National Archives of Australia, Attorney-General’s Department. Cyclone Tracy, Darwin; Australia Government: Canberra, Australia, 2005. [Google Scholar]
- Emlen, J.T. An Urban Bird Community in Tucson, Arizona: Derivation, Structure, Regulation. Condor 1974, 76, 184. [Google Scholar] [CrossRef] [Scilit]
- Chace, J.F.; Walsh, J.J. Urban effects on native avifauna: A review. Landsc. Urban Plan. 2006, 74, 46–69. [Google Scholar] [CrossRef] [Scilit]
- Conole, L.; Kirkpatrick, J. Functional and spatial differentiation of urban bird assemblages at the landscape scale. Landsc. Urban Plan. 2011, 100, 11–23. [Google Scholar] [CrossRef] [Scilit]
- Northern Territory Government. Feral Animals. 2018. Available online: https://nt.gov.au/environment/animals/feral-animals (accessed on 3 October 2018).
- Australian Bureau of Statistics. 2016 Census QuickStats—Darwin. 2016. Available online: http://quickstats.censusdata.abs.gov.au/census_services/getproduct/census/2016/quickstat/701?opendocument (accessed on 27 August 2018).
- Black, D. 1996 Census of Population and Housing: Darwin, a Social Atlas; Statistics, A.B.O., Ed.; Australian Bureau of Statistics: Canberra, Australia, 1997. [Google Scholar]
- Bureau of Meteorology. Climate Statistics for Australian Locations. 2020. Available online: http://www.bom.gov.au/climate/averages/tables/cw_014015.shtml (accessed on 5 July 2020).
- Australian Bureau of Statistics. 3218.0—Regional Population Growth, Australia, 2015–2016. 2016. Available online: http://www.abs.gov.au/ausstats/abs@.nsf/PrimaryMainFeatures/3218.0?OpenDocument (accessed on 9 May 2017).
- Environmental Systems Research Institute (ESRI). ArcGIS 10.4.1 for Desktop, 1999–2015; ESRI: Redlands, CA, USA, 2017. [Google Scholar]
- Conrad, O.; Bechtel, B.; Bock, M.; Dietrich, H.; Fischer, E.; Gerlitz, L.; Wehberg, J.; Wichmann, V.; Böhner, J. System for Automated Geoscientific Analyses (SAGA) v. 2.1.4. Geosci. Model Dev. 2015, 8, 1991–2007. [Google Scholar] [CrossRef] [Scilit]
- Chen, G.; Hay, G.J.; St-Onge, B. A GEOBIA framework to estimate forest parameters from lidar transects, Quickbird imagery and machine learning: A case study in Quebec, Canada. Int. J. Appl. Earth Obs. Geoinf. 2012, 15, 28–37. [Google Scholar] [CrossRef] [Scilit]
- Hay, G.J.; Castilla, G. Geographic Object-Based Image Analysis (GEOBIA): A New Name for a New Discipline. In Object-Based Image Analysis; Springer: Berlin/Heidelberg, Germany, 2008; pp. 75–89. [Google Scholar]
- Fisher, R.P.; Hobgen, S.E.; Haleberek, K.; Sula, N.; Mandaya, I. Satellite Image Analysis and Terrain Modelling-A Practical Manual for Natural Resource Management, Disaster Risk and Development Planning Using Free Geospatial Data and Software. 2017. Available online: https://sagatutorials.wordpress.com/ (accessed on 17 November 2020).
- Australia, B. Birdlife Australia. 2019. Available online: http://birdlife.org.au (accessed on 19 June 2019).
- Atlas of Living Australia. 2019. Available online: https://www.ala.org.au/ (accessed on 1 September 2019).
- Garnett, S.T.; Duursma, D.E.; Ehmke, G.; Guay, P.; Stewart, A.; Szabo, J.K.; Weston, M.A.; Bennett, S.; Crowley, G.M.; Drynan, D.; et al. Australian Bird Data Version 1.0, Figshare, Editor. 2015. Available online: https://doi.org/10.6084/m9.figshare.1499292_D8 (accessed on 10 September 2019).
- Hahs, A.K.; McDonnell, M.J. Selecting independent measures to quantify Melbourne’s urban–rural gradient. Landsc. Urban Plan. 2006, 78, 435–448. [Google Scholar] [CrossRef] [Scilit]
- R Core Team. R: A Language and Environment for Statistical Computing; R Foundation for Statistical Computing: Vienna, Austria, 2019. [Google Scholar]
- Mccrie, N.; Noske, R. Birds of the Darwin Region; CSIRO Publishing: Clayton, Australia, 2015. [Google Scholar]
- Devictor, V.; Julliard, R.; Couvet, D.; Lee, A.; Jiguet, F. Functional Homogenization Effect of Urbanization on Bird Communities. Conserv. Biol. 2007, 21, 741–751. [Google Scholar] [CrossRef] [Scilit]
- Öckinger, E.; Schweiger, O.; Crist, T.O.; Debinski, D.M.; Krauss, J.; Kuussaari, M.; Petersen, J.D.; Pöyry, J.; Settele, J.; Summerville, K.S.; et al. Life-history traits predict species responses to habitat area and isolation: A cross-continental synthesis. Ecol. Lett. 2010, 13, 969–979. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Thomas, C.D. Dispersal and extinction in fragmented landscapes. Proc. R. Soc. B Boil. Sci. 2000, 267, 139–145. [Google Scholar] [CrossRef] [Scilit]
- Slade, E.M.; Merckx, T.; Riutta, T.; Bebber, D.P.; Redhead, D.; Riordan, P.; Macdonald, D.W. Life-history traits and landscape characteristics predict macro-moth responses to forest fragmentation. Ecology 2013, 94, 1519–1530. [Google Scholar] [CrossRef] [Scilit]
- Concepción, E.D.; Moretti, M.; Altermatt, F.; Nobis, M.; Obrist, M.K. Impacts of urbanisation on biodiversity: The role of species mobility, degree of specialisation and spatial scale. Oikos 2015, 124, 1571–1582. [Google Scholar] [CrossRef] [Scilit]
- Parsons, H.; French, K.; Major, R. The influence of remnant bushland on the composition of suburban bird assemblages in Australia. Landsc. Urban Plan. 2003, 66, 43–56. [Google Scholar] [CrossRef] [Scilit]
- Young, K.M.; Daniels, C.B.; Johnston, G. Species of street tree is important for southern hemisphere bird trophic guilds. Austral Ecol. 2007, 32, 541–550. [Google Scholar] [CrossRef] [Scilit]
- Major, R.E.; Parsons, H. What do museum specimens tell us about the impact of urbanisation? A comparison of the recent and historical bird communities of Sydney. Emu Austral Ornithol. 2010, 110, 92–103. [Google Scholar] [CrossRef] [Scilit]
- Kark, S.; Iwaniuk, A.; Schalimtzek, A.; Banker, E. Living in the city: Can anyone become an ‘urban exploiter’? J. Biogeogr. 2007, 34, 638–651. [Google Scholar] [CrossRef] [Scilit]
- McKinney, M.L. Urbanization as a major cause of biotic homogenization. Biol. Conserv. 2006, 127, 247–260. [Google Scholar] [CrossRef] [Scilit]
- Aronson, M.F.J.; La Sorte, F.A.; Nilon, C.H.; Katti, M.; Goddard, M.A.; Lepczyk, C.A.; Warren, P.S.; Williams, N.; Cilliers, S.; Clarkson, B.; et al. A global analysis of the impacts of urbanization on bird and plant diversity reveals key anthropogenic drivers. Proc. R. Soc. B Boil. Sci. 2014, 281, 20133330. [Google Scholar] [CrossRef] [Scilit]
- Sol, D.; Bartomeus, I.; González-Lagos, C.; Pavoine, S. Urbanisation and the loss of phylogenetic diversity in birds. Ecol. Lett. 2017, 20, 721–729. [Google Scholar] [CrossRef] [Scilit]
- Parks and Wildlife Commission of the Northern Territory. Feral Pigeon Eradication Program: Darwin 1997; Parks and Wildlife Commission of the Northern Territory: Darwin, Australia, 1998. [Google Scholar]
- ABC Darwin. Darwin Eradicates Feral Pigeons; ABC Darwin: Darwin, Australia, 2004. [Google Scholar]
- NAFI: North Australia and Rangelands Fire Information. 2018. Available online: https://www.firenorth.org.au/nafi3/ (accessed on 8 January 2019).
- Bowman, D.M.; Johnston, F.H. Wildfire Smoke, Fire Management, and Human Health. EcoHealth 2005, 2, 76–80. [Google Scholar] [CrossRef] [Scilit]
- Johnston, F.H.; Hanigan, I.C.; Bowman, D.M.J.S. Pollen Loads and Allergic Rhinitis in Darwin, Australia: A Potential Health Outcome of the Grass-Fire Cycle. EcoHealth 2009, 6, 99–108. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- USGS. What are the Band Designations for the Landsat Satellites? 2020. Available online: https://www.usgs.gov/faqs/what-are-band-designations-landsat-satellites?qt-news_science_products=0#qt-news_science_products (accessed on 17 November 2020).
- USGS. What are the Best Landsat Spectral Bands for Use in My Research? 2020. Available online: https://www.usgs.gov/faqs/what-are-best-landsat-spectral-bands-use-my-research?qt-news_science_products=0#qt-news_science_products (accessed on 17 November 2020).

Publisher’s Note: MDPI stays neutral with regard to jurisdictional claims in published maps and institutional affiliations. |
© 2021 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).