


Highlights
- This study presents the first inventory of soil bacterial communities using metagenomic analysis in the Lower-Chéliff Plain, showing high bacterial diversity and a community dominated by Actinomycetota and Pseudomonadota.
- Reduced tillage with Cover Crop and cultivator operations combined with organic fertilization is needed in the Lower-Chéliff Plain to improve soil fertility, nutrient availability, and microbial biodiversity.
- Tillage and fertilizer treatments had significant effects on the availability of soil nutrients and bacterial community structure. Among the mineral elements, phosphorus varied most significantly. Tillage affected bacterial diversity more than fertilization, while dominant bacterial phyla were relatively stable among the different soil practices.
Abstract
This study examines the effects of fertilizer amendment type and tillage practice on soil chemical properties and bacterial community, as biological indicators of soil fertility, with the aim of conserving this biological system in agro-ecosystem production contexts. In the experiment, conventional tillage (CT) was compared with three (3) minimum tillage (MT) methods. Metagenomic analysis was performed to determine the bacterial community composition at the phylum level. The treatments had the greatest impacts on phosphorus (P) dynamics, while other mineral elements remained relatively stable due to differences in nutrient availability mechanisms. The results revealed similarities between different treatments, particularly between minimum tillage (MT) with the same mineral (M) input as well as between treatments using organic (O) inputs, while CT with mineral input appeared to be the most distinct. Tillage has a small but statistically significant structural impact on the configuration of microbial communities (p-Value < 0.05) in terms of major bacterial phyla. In this analysis, the Shannon index varied between 5.48 and 5.23, indicating a particularly diverse bacterial community characteristic of agricultural soils with significant biological activity. Bacteria of the phyla Planctomycetota and Verrucomicrobiota were found to correlate positively with those of the Actinomycetota phylum, which are considered beneficial bacteria. Thus, such bacteria may serve as biological indicators of agricultural soil bio-fertility. The study’s results demonstrate that tillage seems to have a greater impact on bacterial diversity than fertilization; in this regard, reduced tillage using a combination of two implements (cover crop incorporation and a tine cultivator) is suggested as the most suitable option for the type of soil considered in this study.
1. Introduction
1.1. Mineral Elements in Cultivated Soils
Mineral elements originating from the soil are vital nutritional sources for plants, due to their involvement in a large number of physiological processes. A distinction is generally made between macronutrients and micronutrients, which are essential for normal plant growth [1].
Among the nutrients that are necessary for growth, the essential nutrients (e.g., nitrogen (N), phosphorus (P), and potassium (K)) are often of mineral origin, with their availability influenced by microbial activity. Conversely, microelements such as manganese (Mg) and iron (Fe), which are necessary for enzymatic activity and photosynthesis, are often limiting due to their immobilization in insoluble mineral complexes in the soil [2]. Iron—one of the most limiting trace elements—is involved in chlorophyll synthesis and the activation of enzymes, making the presence of iron-solubilizing bacteria in the soil important to compensate for these deficiencies.
Soil bacteria, fungi, actinomycetes, protozoa, nematodes, and algae make up the soil microbial community known as soil microbiota. Soil microorganisms, the presence of which depends on the age and type of the soil, play crucial roles in soil fertility and are considered bioindicators of biological and chemical parameters of the soil [3].
The soil bacterial community has garnered considerable research interest relating to biological processes, including organic matter (OM) decomposition, and plays critical roles in agricultural soil management systems [4].
1.2. Role of Bacteria in the Soil
Bacteria and their diversity also play roles in the cycling of nutrients. Nitrogen fixation is a process that is carried out by certain N-fixing bacterial species, such as those of the genus Rhizobium‚ which live symbiotically with the roots of legumes and assimilate atmospheric N in a form that is usable by plants‚ allowing for decreased application of mineral amendments [5].
Other helpful soil microbes, including those of the genera Azotobacter and Bacillus, can also fix N naturally in the soil‚ as well as solubilize phosphorus (P) and potassium (K)‚ thus making them available for absorption by plant roots [6].
Most OM decomposition is performed by soil bacteria, including Actinomycetes. Some Actinomycetes can survive in highly alkaline conditions‚ and can break down dead and decaying matter into elements that can then be absorbed by plants. Soil bacteria make important contributions to maintaining soil fertility through the leaching of nutrients from the soil, which is particularly important for nutrient cycling [7].
Soil bacteria can also help to remove pollutants from the environment by converting them to non-toxic compounds [8]. Soil microorganisms also play an active role in regulating plant-available nutrients in the soil; for instance‚ zinc-solubilizing soil bacteria secrete organic acids that can effectively liberate zinc from soil minerals, increasing its availability for zinc-deficient plants such as wheat [9].
1.3. Interactions Between Minerals and Groups of Microorganisms
The interactions between mineral nutrients and microbial populations are key elements of dynamic soil systems characterized by soil fertility and nutrient cycling. The biogeochemical process of microbial mineralization of soil leads to the dissolution of minerals, which causes enrichment of the soil solution in both major and minor nutrients [10].
Minerals are released from parent rock through weathering and, when combined with microbial inoculants, can improve soil fertility and nutrient availability for crops. Bacteria play a crucial role in altering the soil’s mineral composition and can influence soil properties and dynamics. The effectiveness of these bacterial functions depends on diverse factors, such as the soil type, soil microbial composition, and environmental conditions [11]. Previous research on how tillage affects soil fauna has shown that it frequently disturbs a wide variety of organisms, ranging from microscopic bacteria and fungi to large burrowing animals such as moles and predators such as snakes [12].
Soil tillage is a cultivation practice that involves the use of machines to prepare the soil for seeding, and its effects on soil fertility and crop yields can be both significant and complex. Tillage-related methods include conventional tillage, no-till conservation agriculture, and direct seeding, each having very different effects on the soil’s physico-chemical properties, its capacity to make various nutrients available to plants, and the structure and diversity of the microbial communities that inhabit it [13].
The effects of tillage on mineral dynamics and the bacterial community are significant. Traditional (conventional) tillage destroys the soil structure, often leading to decreases in biomass and microbial biodiversity, along with impaired nutrient availability and soil fertility [14].
Soil conservation procedures such as no-till farming have been shown to increase the diversity of bacteria and nutrient availability by means of soil structure and OM improvements. These practices are considered sustainable, soil-enhancing, and capable of reducing environmental degradation [15].
The effects of tillage on the bioavailability of mineral nutrients and soil bacteria have also been studied. The disadvantages of tillage include soil erosion, decreased OM, and degradation of soil health in the case of plowing, while its advantages lie in weed control and adequate seedbed preparation [16]. Meanwhile, practitioners of reduced tillage and no-till farming have argued that these practices could, in the long term, increase soil microbiome resilience and nutrient cycling, thus presenting them as sustainable agricultural practices that promote soil health and a more balanced ecosystem [17].
According to Wang et al. (2017) [18], agricultural land management and technical practices can affect soil microbial diversity; for example, in one study, tillage increased microbial diversity in soils. This may mean that a lower level of disturbance allows for the establishment of greater bacterial species diversity and better ecosystem functioning, whereas a higher level of disturbance (e.g., intensive soil tillage) could diminish microbial diversity, consequently having an impact on the health and productivity of soil [19].
2. Materials and Methods
The experimental protocol was implemented at a university experimental station in 2024 at the following geographical coordinates:
Latitude 36°11′19″ N, Longitude 1°14′56.6″ E, Altitude 100 m.
The experimental plot is situated on the Bas-Chéliff plain, Algeria, which consists mainly of alluvial deposits. The agricultural soils of the Bas-Chéliff plain are predominantly clayey and heavy, characterized by a high proportion of fine-textured material and widespread salinity problems [20].
The experiment aimed to analyze the influence of four (4) tillage techniques (conventional tillage and three minimum tillage techniques) combined with organic and/or mineral treatments on soil chemical status and microbial diversity, serving as indicators of soil fertility. A randomized complete block design (RCBD) with three (3) replications was conducted.
Plowing was carried out in November of 2023 at the experimental station using a reversible-blade plow. Simplified tillage operations were performed two months later (mid-January 2024) under moderate moisture conditions. Each experimental plot was divided into four (4) micro-plots width-wise. To assess the effects of the four cultivation techniques (T), we selected the treatments listed in Table 1 below.
Table 1.
Different tools used in cultivation practices.
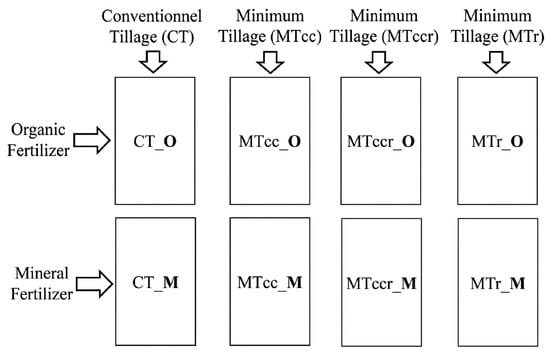
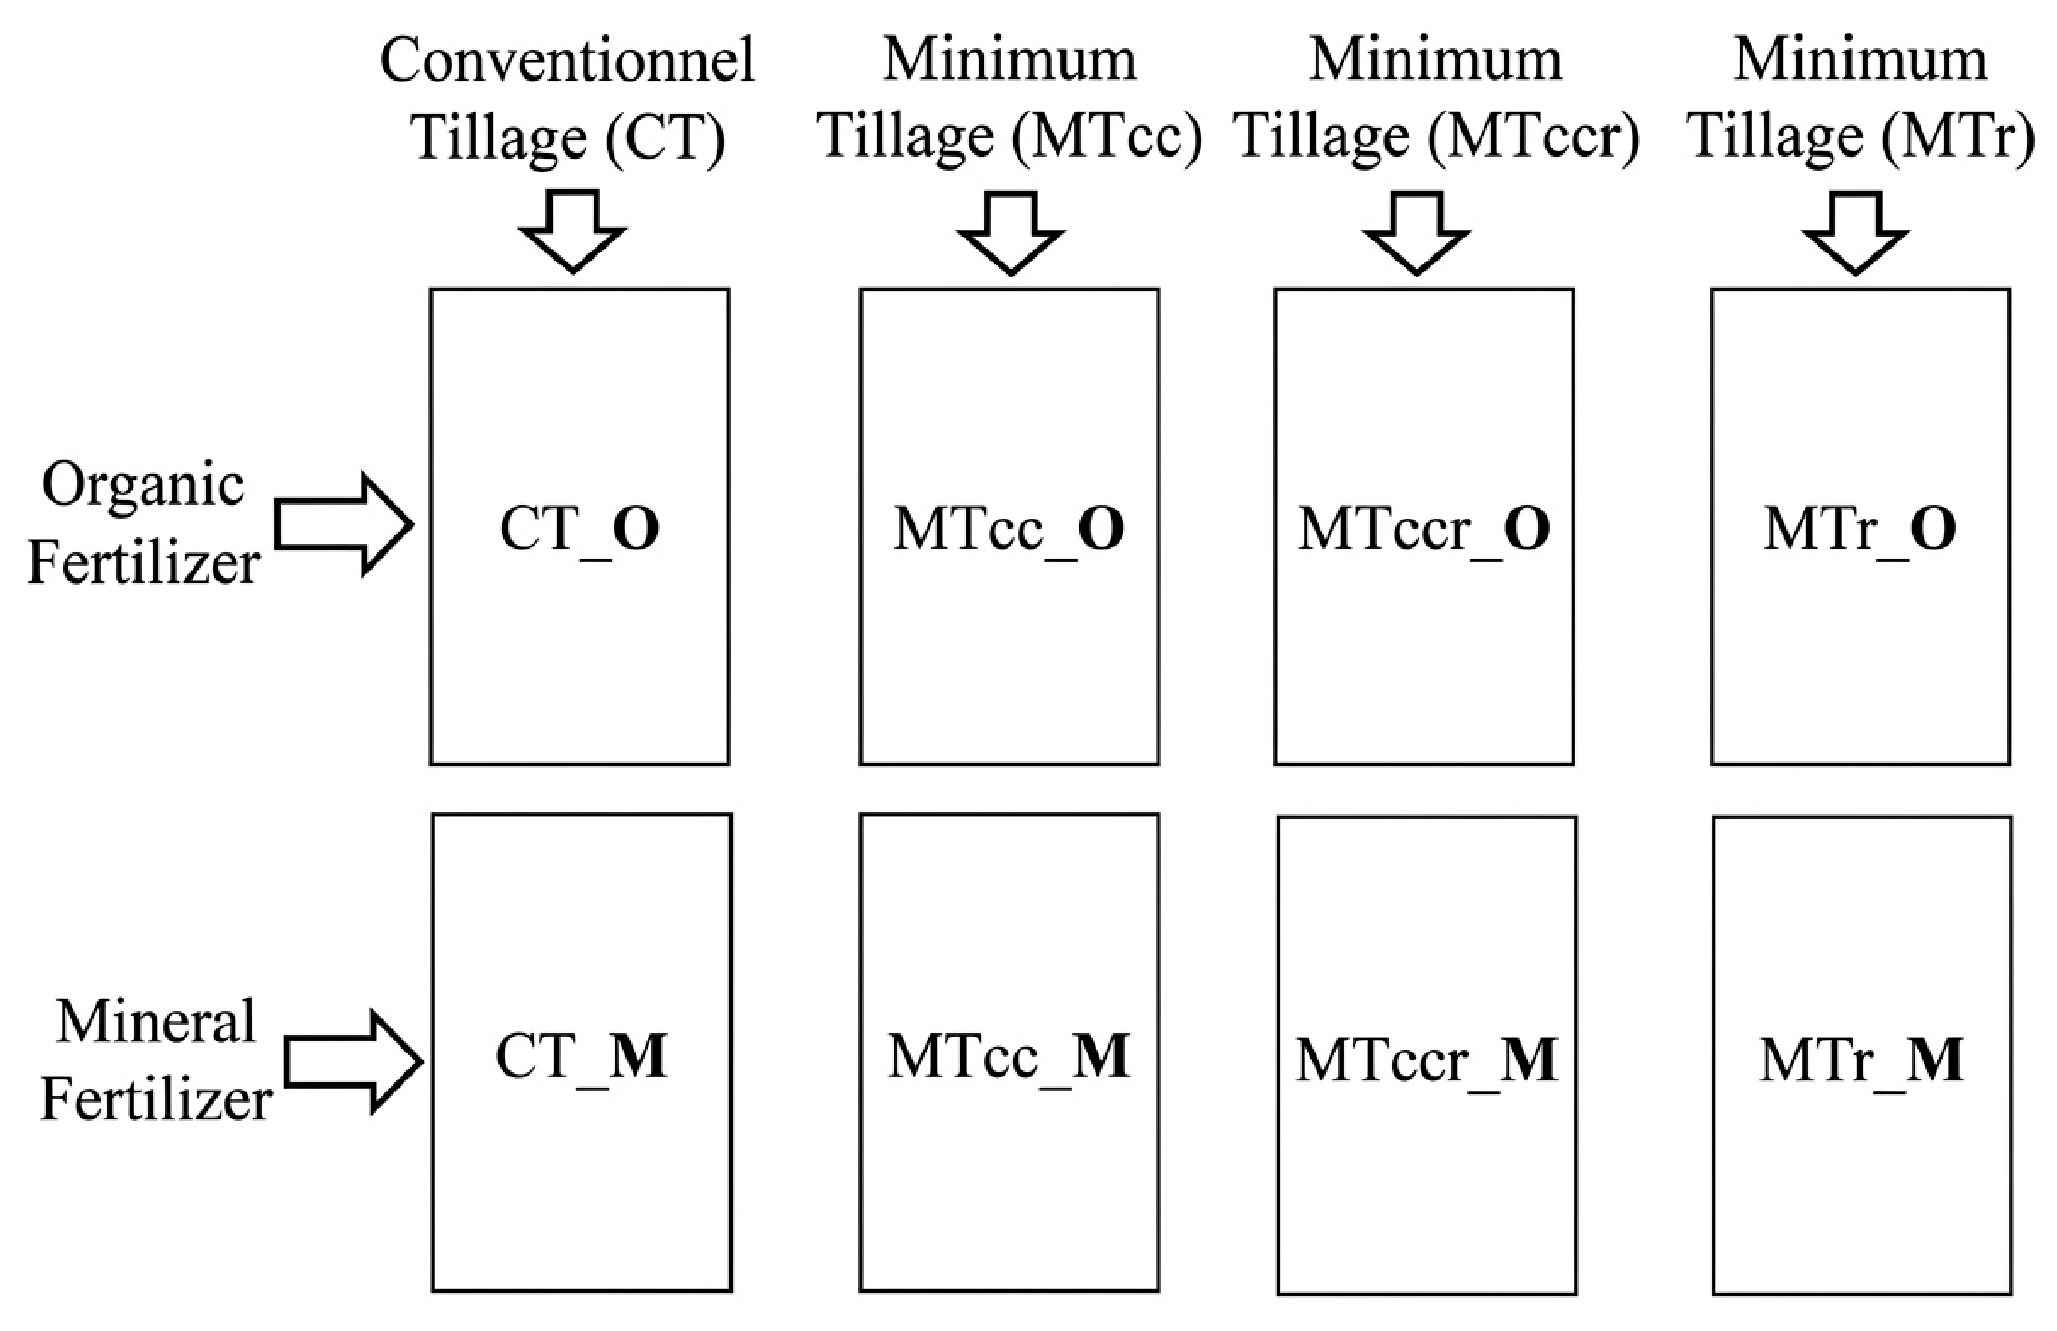
The dimensions of each micro-plot were as follows: Length, 15 m; width, 3 m. Each micro-plot was split into two, each with one of two amendment types, namely organic (O) fertilizer from sheep manure or 15-15-15 mineral (M) fertilizer. As a result, there were eight micro-plots in each experimental plot. The soil was analyzed using an experimental apparatus prior to seeding, serving as a control reference.
In Figure 1, the treatments were organized in this way to limit the number of tractor passes to a single operation, for both tilling the soil and applying fertilizer. The micro-plots were cultivated with chickpea in February of 2024. Irrigation was carried out using a controlled sprinkler irrigation system, which allowed the irrigation dose to be accurately regulated for each experimental treatment. The amount of water applied was controlled to minimize excessive water application and, consequently, the risk of surface runoff between adjacent plots. Therefore, irrigation was managed to avoid significant water transfer from one plot to another.
Figure 1.
Diagram of a block of the experimental set-up.
2.1. Soil Chemical Analysis
Soil samples were collected from several sampling points within each plot in mid-May of 2024, then thoroughly mixed to obtain a homogeneous composite sample. The composite sample was then spread on a clean surface, divided into four equal portions, and two opposite quarters were discarded. The remaining soil was remixed, and the quartering procedure was repeated until the amount of soil required for laboratory analysis was obtained, following ISO 18400-201:2017 [21].
Once a site was selected for assessment‚ samples were collected using sterile tools to avoid contamination‚ then dried and ground into a fine powder. We took three (3) random samples from each micro-plot, resulting in a total of nine (9) samples for each treatment. The samples were then ground and passed through a predetermined series of screens, such that all particle fractions in the sample to be analyzed were of the same size, thus providing accurate results.
Laboratory analysis was performed using the following procedures:
Determination of organic carbon (OC) and total carbon (C) was carried out according to ISO-10694. Nitrogen (N) was measured according to ISO-13878, using the dry combustion method with digestion at 420 °C, followed by distillation and titration [2].
For determination of organic matter (OM), 1 g of soil was weighed, to which 10 mL of dichromate (K2Cr2O7 1N) and 20 mL of sulfuric acid (H2SO4) were added [22]. The mixture was left to react for 30 min, then distilled and titrated with ferrous sulfate (FeSO4).
Determination of assimilable phosphorus (P) was achieved by shaking 2.5 g of soil with 50 mL of 0.5 M NaHCO3 (pH 8.5) for 30 min, followed by using a spectrophotometer at 882 nm according to the Olsen method [22].
For determination of exchangeable cations, 5 g of the soil and 100 mL of ammonium acetate were stirred for one (1) hour. Then, measurements were performed using an Atomic Absorption Spectrometer. This test allows for the measurement of potassium (K), calcium (Ca), magnesium (Mg), and sodium (Na).
2.2. Microbial Diversity Analysis
Eight (8) samples were submitted for LEM Metagenomic sequencing at IRDA. A FastDNA SPIN kit was employed for total genomic DNA isolation from the soil samples (MP Biomedicals, Solon, OH, USA), in accordance with the manufacturer’s instructions. For effective lysis of microorganisms found in soil samples, the kit involves mechanical disruption using Lysing Matrix E tubes and a FastPrep device. The kit’s silica-based Binding Matrix and SPIN filter process were then used to purify the extracted DNA.
The laboratory within the Institute for Research in Construction (IRDA)—a specialized Microbial Ecology Laboratory located in Quebec, Quebec, Canada—carried out amplicon sequencing library preparation and bioinformatics analysis of the DNA sequences. Illumina MiSeq 2 × 300 bp sequencing was conducted as part of the genomic data analysis workflow of the Institute for Integrative Biology and Systems (IBS) at Laval University (Quebec, Canada).
Spectrophotometry was performed to quantify the absorbance values at 260 and 280 nm, thus also providing the A260/A280 ratio, in order to assess the amount and quality of the purified genomic DNA.
Metagenomic evaluations were conducted to examine the variety of prokaryotes (archaea and bacteria). PCR amplification of the V4 hypervariable region of the 16S ribosomal RNA (rRNA) gene from prokaryote organisms was carried out with the region-specific primers described by Lewis et al. [23], using a dual-indexed PCR approach (two-step PCR approach, The primer pair consisted of 515F-Y (5′-GTGYCAGCMGCCGCGGTAA-3′), and 806R-AG (5′-GGACTACNVGGGTWTCTAAT-3′),) specially designed for analyses using the Illumina MiSeq (high-throughput sequencing platform).
Amplification of the bacterial V4 region of 16S ribosomal DNA was performed in 25 μL reactions containing 1 to 10 ng of genomic DNA‚ 0.2 μM degenerate forward and reverse primers (515F-Y and 806R-AG)‚ and other reagents in a high-fidelity PCR master mix. Cycling parameters included an initial denaturation step at 94 °C for 3 min and 30 cycles at 94 °C for 45 s‚ 50 °C for a 60 s primer annealing step‚ and 72 °C for a 90 s extension step. A 10 min final extension step at 72 °C completed amplification. Samples were run on an agarose gel before sequencing.
The amplicon libraries were sequenced in paired-end format with a 300-base read (i.e., 2 × 300 base pairs (bp) on each side of the DNA) sequencing-stranded protocol on the Illumina MiSeq system at the genomic analysis laboratory of Laval University (Quebec, CA) in the Institute of Biology and Integrative Systems (IBIS).
The bacterial community’s diversity was assessed using the Shannon diversity index (H’), as defined in Equation 1, which was also applied in the authors’ previous study [24].
where Ni is the number of individuals of species i and N is the total number of specimens from all species in the samples (Table S1: taxonomy).
An H’ value less than 2 indicates low diversity; an H’ value between 2 and 4 indicates moderate diversity; and an H’ value greater than 4 indicates high diversity of a bacterial assemblage.
Sequence bioinformatics analyses were conducted using the bioinformatics platform of the LEM at the IRDA, which involved disparate processing strategies implemented via Qiime2 according to Bolyen et al. [25], including procedure quality validation, reference databases, and calculation of indices for microbial diversity comparisons after measuring microbial richness. The Greengenes 13.8 reference database was employed for taxonomic assignment of the identified genetic variants [26].
2.3. Statistical Analyses and Processing of Data
All data were processed using the OriginLab 2019b Corporation software (version 9.6.5.169) and are presented as mean ± standard error (SE). One-way ANOVA was utilized to evaluate statistically significant differences between parameters analyzed under different soil tillage practices. Two-way ANOVA was performed to determine the interactions and main effects of fertilizer and soil tillage on mineral nutrients and bacterial heterogeneity. Tukey’s post hoc test (p-value < 0.05) was utilized for multiple comparisons. Principal Component Analysis (PCA) of the resulting data was performed with the same software in order to establish the correlations between bacterial phyla and to determine the homogeneous groups between the treatments.
3. Results
3.1. Impact of Treatment on the Soil Nutrients
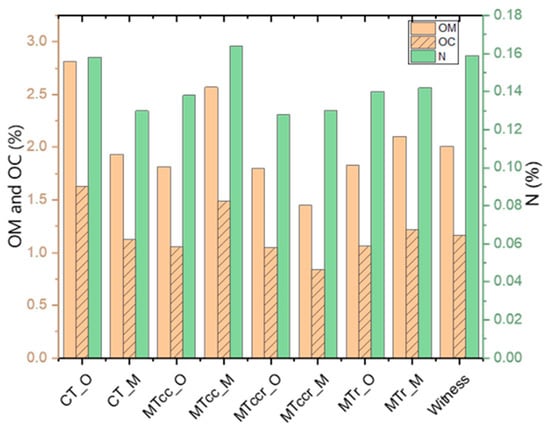
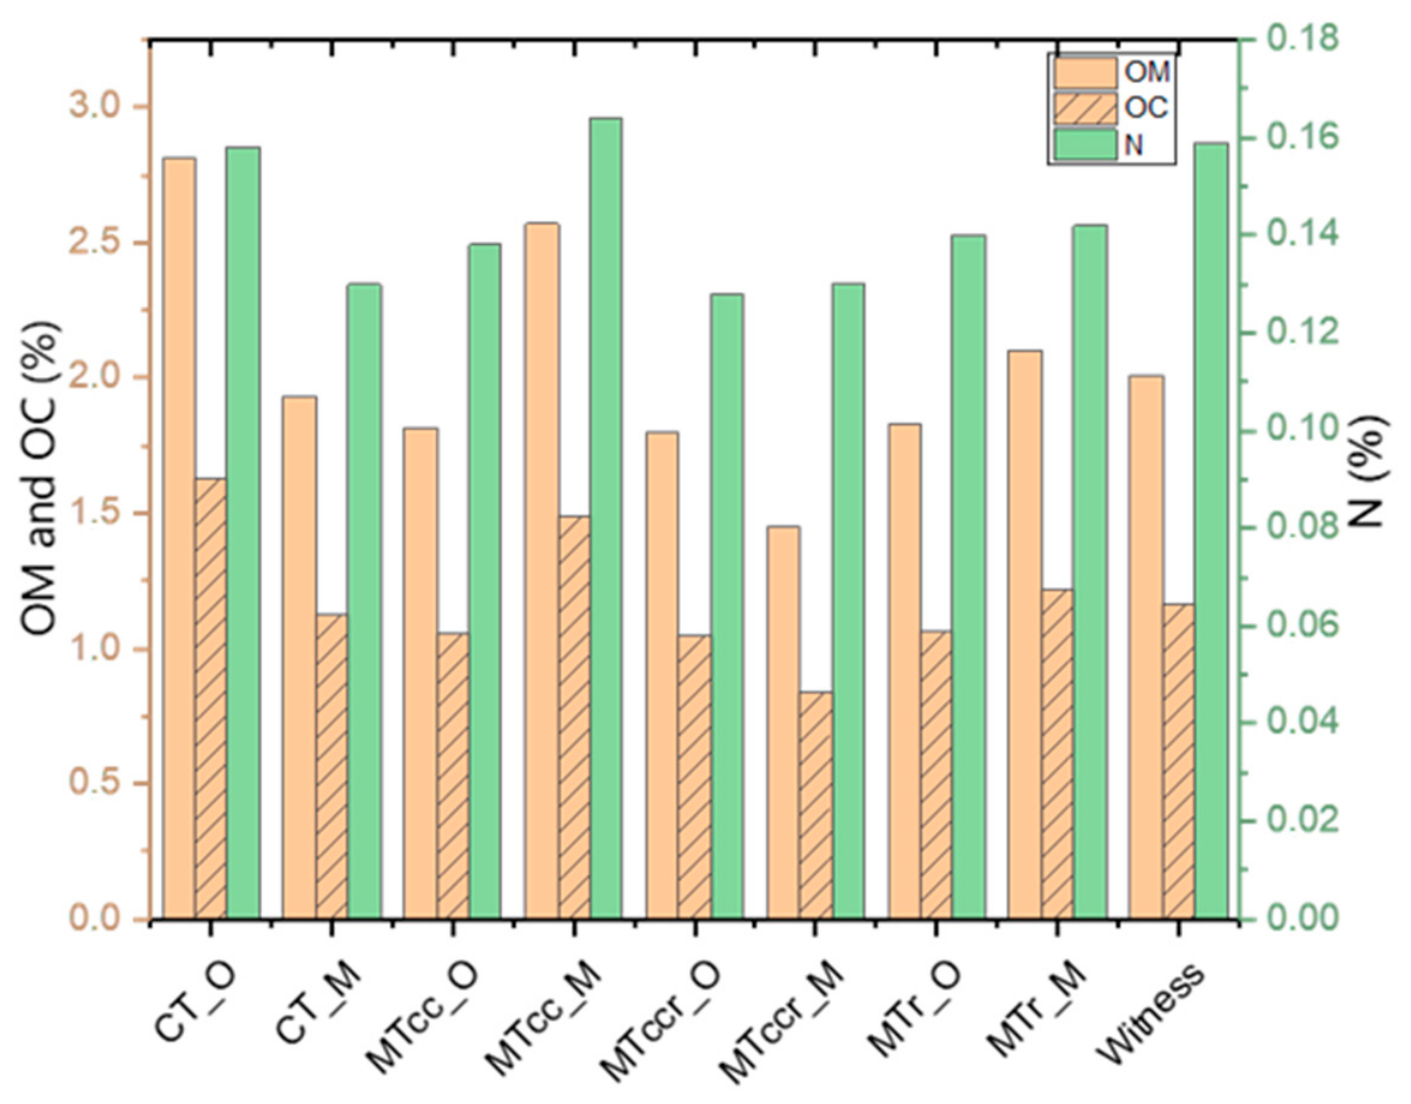
Figure 2 presents the impacts of fertilizer and tillage treatments on the percentages of organic carbon (OC), nitrogen (N), and organic matter (OM) in the soil. Soil organic matter (OM) enhances the chemical properties of the soil, allowing plants—both cultivated and wild—to grow healthily.
Figure 2.
Impacts of fertilizer and tillage on organic matter (OM), nitrogen (N), and organic carbon (OC) in the soil. CT: Conventional tillage; MTcc: Minimum tillage with cover crop; MTr: Minimum tillage with cultivator; MTccr: Minimum tillage combine cover crop and cultivator; O: organic fertilizer; M: mineral fertilizer.
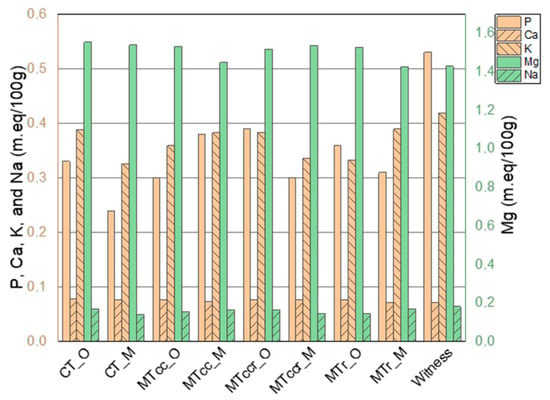
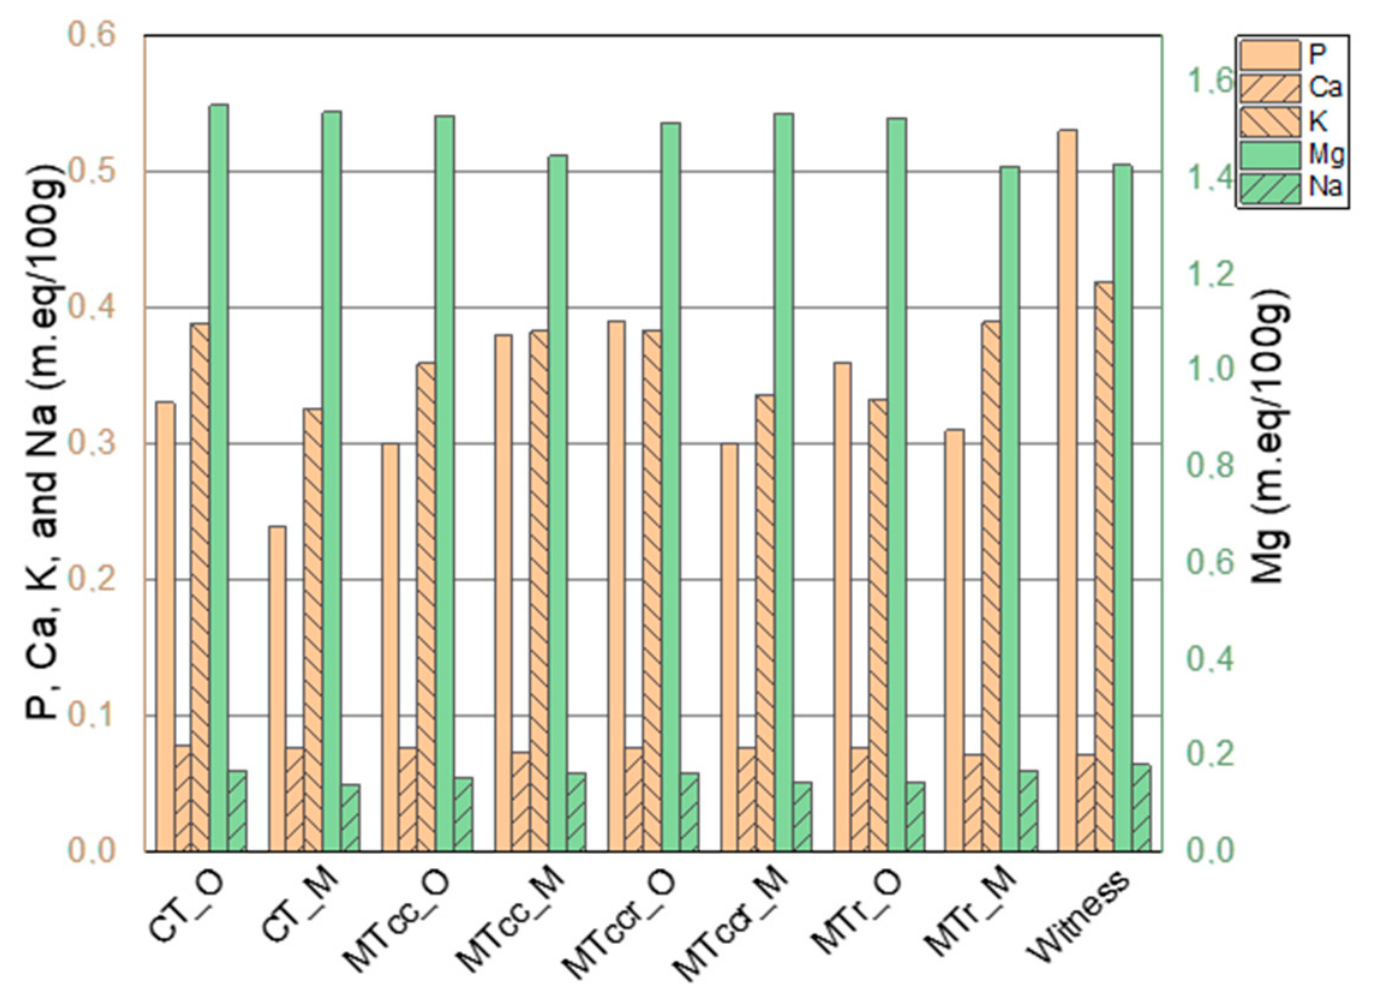
The soil levels of the five minerals (P, Ca, K, Mg, and Na) under the different treatments used are summarized in Figure 3. For some elements, variations can be observed between treatments, while for others, the concentrations remain constant across all treatments. Magnesium (Mg) was an abundant element under all treatments, with only a slight difference between the treatments—ranging from 1.45 to 1.60 m.eq/100 g (right axis)—indicating that the magnesium concentration is relatively constant.
Figure 3.
Impact of treatments on the elements P, Ca, K, Na, and Mg in m.eq per 100 g. CT: Conventional tillage; MTcc: Minimum tillage with cover crop; MTr: Minimum tillage with cultivator; MTccr: Minimum tillage combine cover crop and cultivator; O: organic fertilizer; M: mineral fertilizer.
The effects of treatment were strongest for P, which was highly variable; as such, P absorbance is likely most affected by treatment, due to its variance in availability. The concentrations of K‚ Ca‚ and Na were relatively similar and did not vary greatly among treatments, which may indicate that they are less affected by soil tillage or fertilizer category, or that their native soil reserves are large enough to mask the effects of the treatment.
For phosphorus (P)—the nutrient whose levels varied the most between treatments—its concentration in the soil ranged from 0.24 to 0.53 m.eq/100 g (left axis), with levels lower than the initial value (i.e., before sowing). Potassium (K) had intermediate concentrations of approximately 0.30 to 0.42 m.eq/100 g, which varied moderately from one treatment to another. Calcium (Ca) was present in very small amounts (0.06 to 0.08 m.eq/100 g), and its presence varied little from one treatment to another. Similarly, the concentration of sodium (Na)—which was the least abundant element—was close to zero for all treatments and did not vary much.
3.2. Metagenomic Analysis of the Soil Bacteria Phyla Abundance
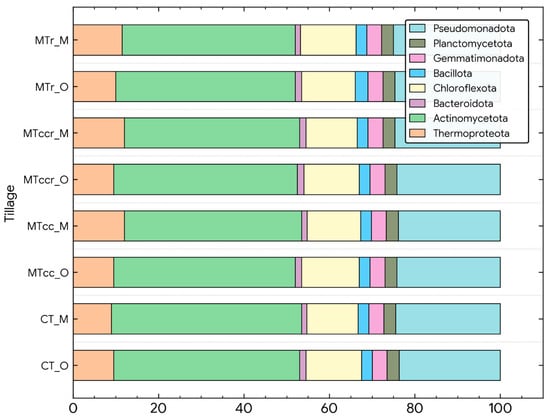
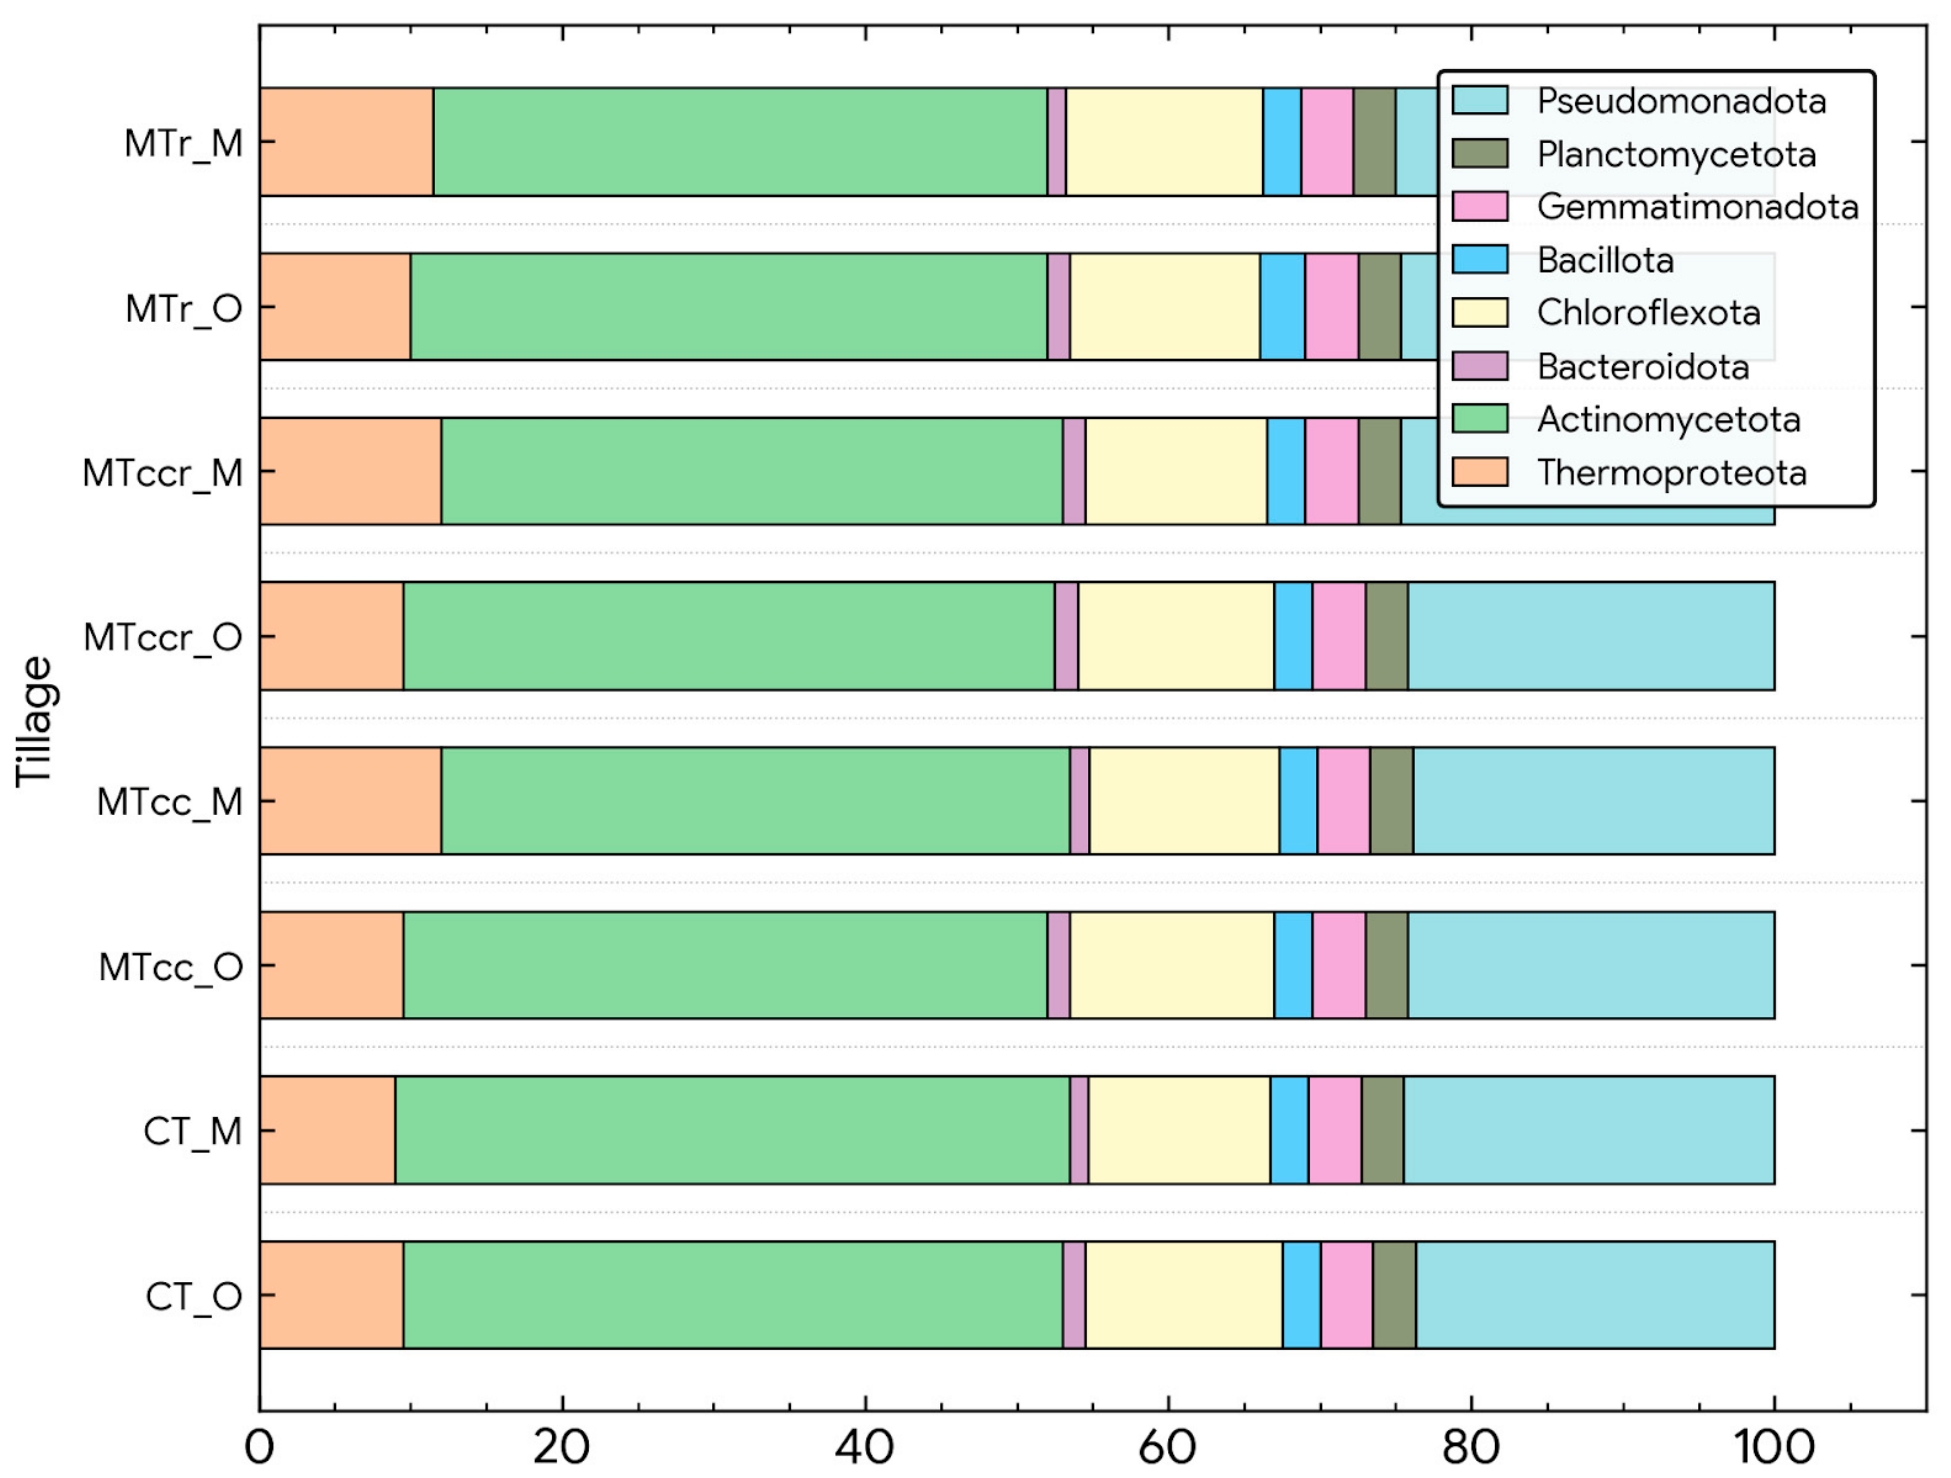
The relative abundances of the main soil bacterial phyla under the tillage systems CT, MT_cc, MT_ccr, and MT_r and different fertilizer applications (M and O) are presented in Figure 4. All treatments had a comparatively consistent bacterial community structure, although the relative abundances of some phyla varied between the soil treatments.
Figure 4.
Relative abundance of bacterial community in each tillage treatment. CT: Conventional tillage; MTcc: Minimum tillage with cover crop; MTr: Minimum tillage with cultivator; MTccr: Minimum tillage combine cover crop and cultivator; O: organic fertilizer; M: mineral fertilizer.
Actinomycetota represented a large proportion of the phyla regardless of the treatment, with percentages ranging from 42% to 46%. The maximum value of 46% was observed under conventional tillage with mineral application (CT_M). For the other treatments, the values varied between 42% and 44%. Despite these relative differences in abundance, the distribution of Actinomycetota remained relatively stable across treatments.
In terms of quantity, the next most represented phylum was Pseudomonadota, with proportions varying between 22 and 24% depending on the treatment, with the highest proportions achieved under the MTr_O and MTcc_O treatments. Given these similarities, we can deduce that the bacterial community composition is relatively stable. The phylum Thermoproteota, which ranked third in terms of relative abundance, represented only 9 to 12% of the sequences; in particular, it reached 9% under the CT_M tilled soil treatment and 10 to 12% under the other treatments.
The phylum Chloroflexota had the most consistent abundance (12–13%) across treatments. The phyla Gemmatimonadota and Bacillota each constituted 4 to 5% of the bacterial community, while the phyla Planctomycetota and Bacteroidota represented only 1 to 2% of the bacterial community.
In conclusion, these results demonstrate that the soil bacterial community is largely dominated by Actinomycetota and Pseudomonadota in tilled soils (CT), while the other phyla remain relatively stable. The different tillage treatments induced only slight variations in the relative abundances of the main phyla.
3.3. Statistical Analysis of the Effect of Treatment on the Soil Fertility Indicators
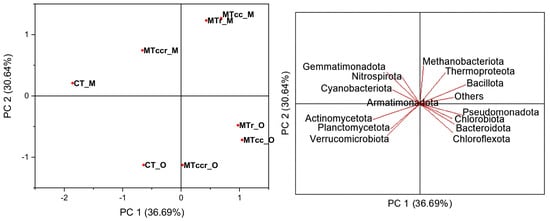
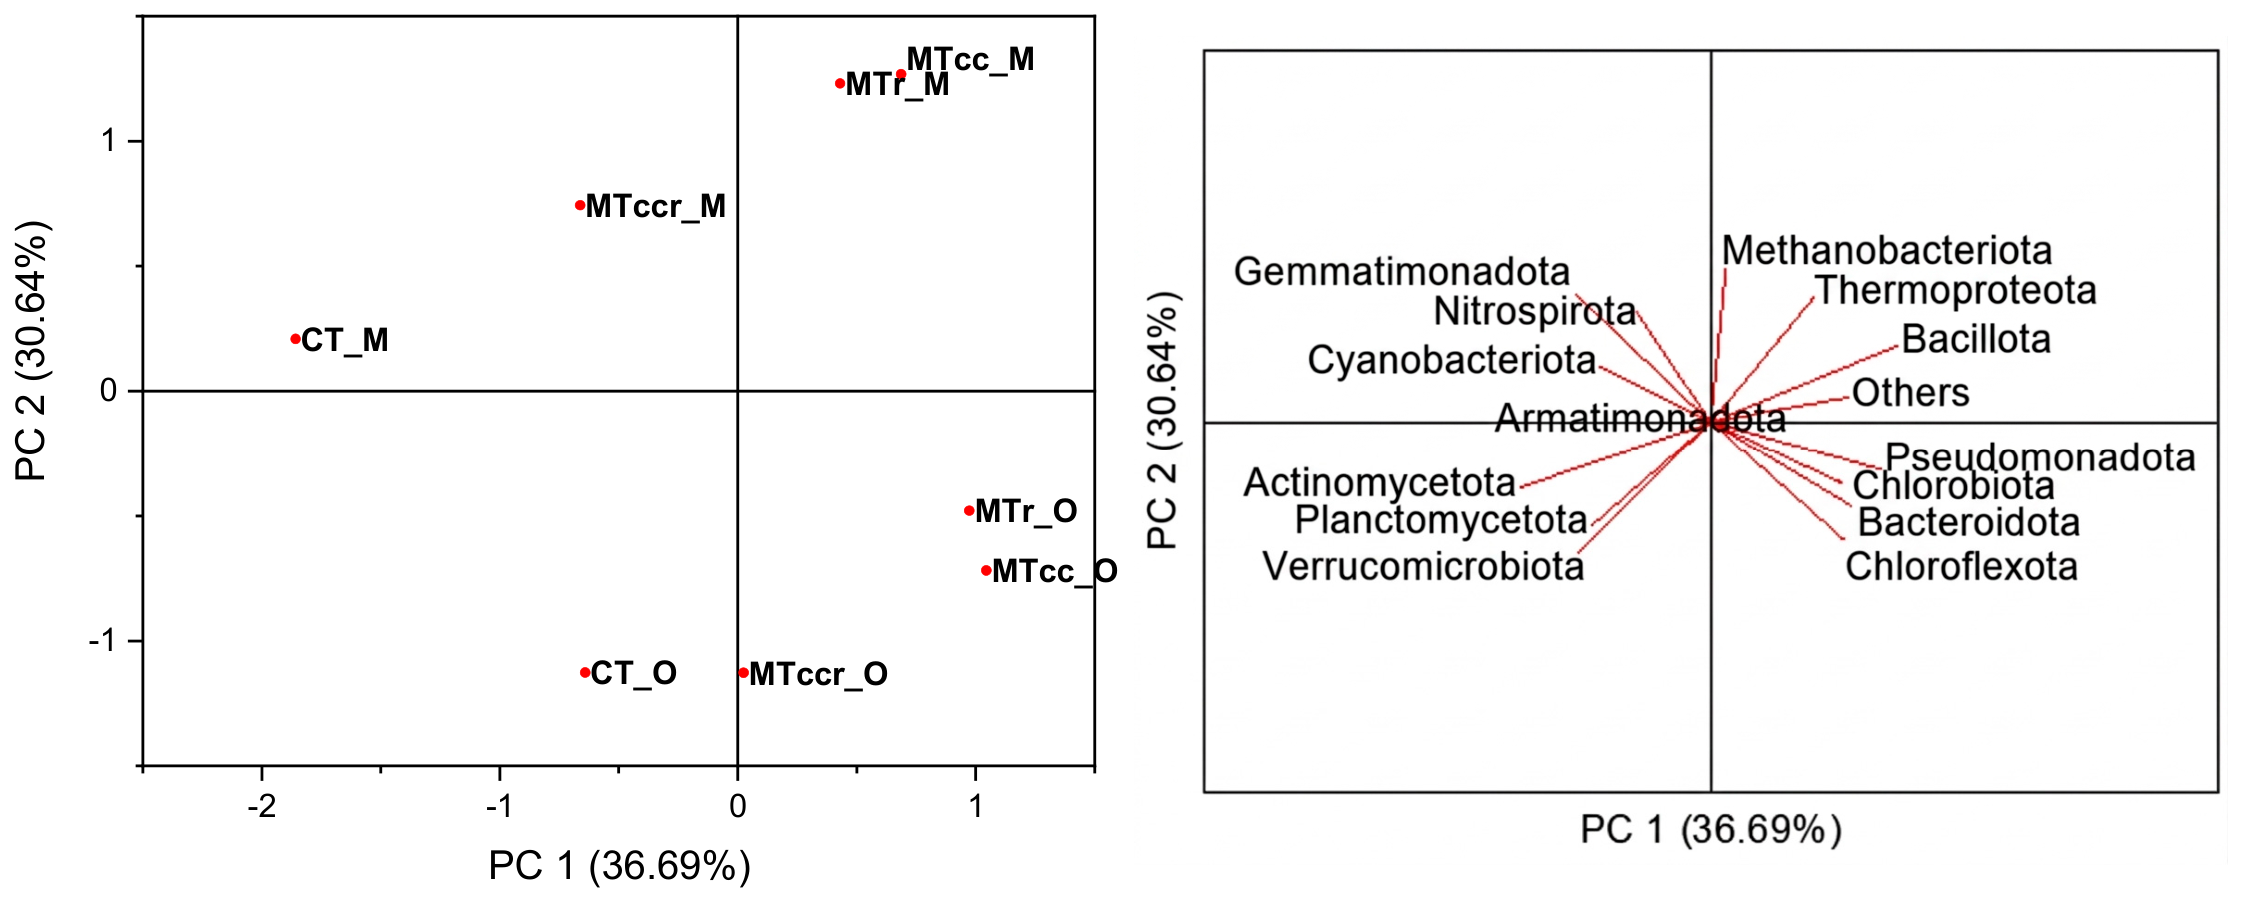
From the Principal Component Analysis (PCA) results shown in Figure 5, it can be seen that the first two axes explain 67.33% of the observed variation (36.69% for PC1 and 30.64% for PC2). This proportion of variance is a relatively large proportion of the total variance in bacterial phylum composition across the treated soils.
Figure 5.
PCA ordination plot, allowing for comparison of the soil diversity under each treatment. CT: Conventional tillage; MTcc: Minimum tillage with cover crop; MTr: Minimum tillage with cultivator; MTccr: Minimum tillage combine cover crop and cultivator; O: organic fertilizer; M: mineral fertilizer.
The PC1 axis is correlated positively with Pseudomonadota, Chloroflexota, Bacteroidota, Chlorobiota and, to a lesser extent, Bacillota, and negatively associated with Actinomycetota, Planctomycetota, Verrucomicrobiota, Gemmatimonadota, and Cyanobacteriota.
In the PC2 axis, the contributions of the phyla Methanobacteriota, Nitrospirota, Thermoproteota, and Bacillota are positive, while those of Chloroflexota, Bacteroidota, Pseudomonadota, Actinomycetota, and Verrucomicrobiota are negative. Phyla near the center of the graph, such as Armatimonadetes, make only a small contribution to the separation in the main components.
It can also be observed that the MTr_M and MTcc_M treatments, which use only one tool and the same type of fertilizer, are very close to each other. Similarly, the MTr_O and MTcc_O tillage techniques also form a relatively close group, reflecting the comparable microbial composition under these two treatments in terms of the considered organisms.
The minimum tillage treatment (MTccr_M) with mineral (M) fertilizer can be seen to occupy an intermediate position within the groups located in the upper right part, as well as with the CT_M treatment of the soil.
Finally, it is worth noting that conventional tillage (CT_O) and reduced tillage (MTccr_O)—which both use two implements and induce intensive soil use—were located in the lower quadrants. This analysis explicitly reveals a bacterial composition that differs from that of the treatments located in the upper half of the graph; however, the distances between the various treatments remain minimal.
The analysis of variance (ANOVA) results for the obtained data are summarized in Table 2, from which it can be seen that both tillage and fertilization have a statistically significant influence on all measured properties (i.e., soil bacteria, mineral N, P, and K). Both factors were found to significantly affect the presence and amount of available nutrients within the soil matrix, as well as influencing the abundance and type of microorganisms present. Statistically, the treatment means were found to fluctuate (p < 0.05), making it highly improbable that these observed differences were due to chance.
Table 2.
Two-way ANOVA for bioindicators of bio-fertility of soil.
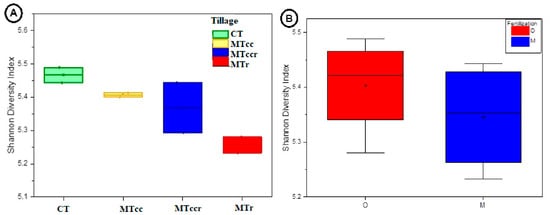
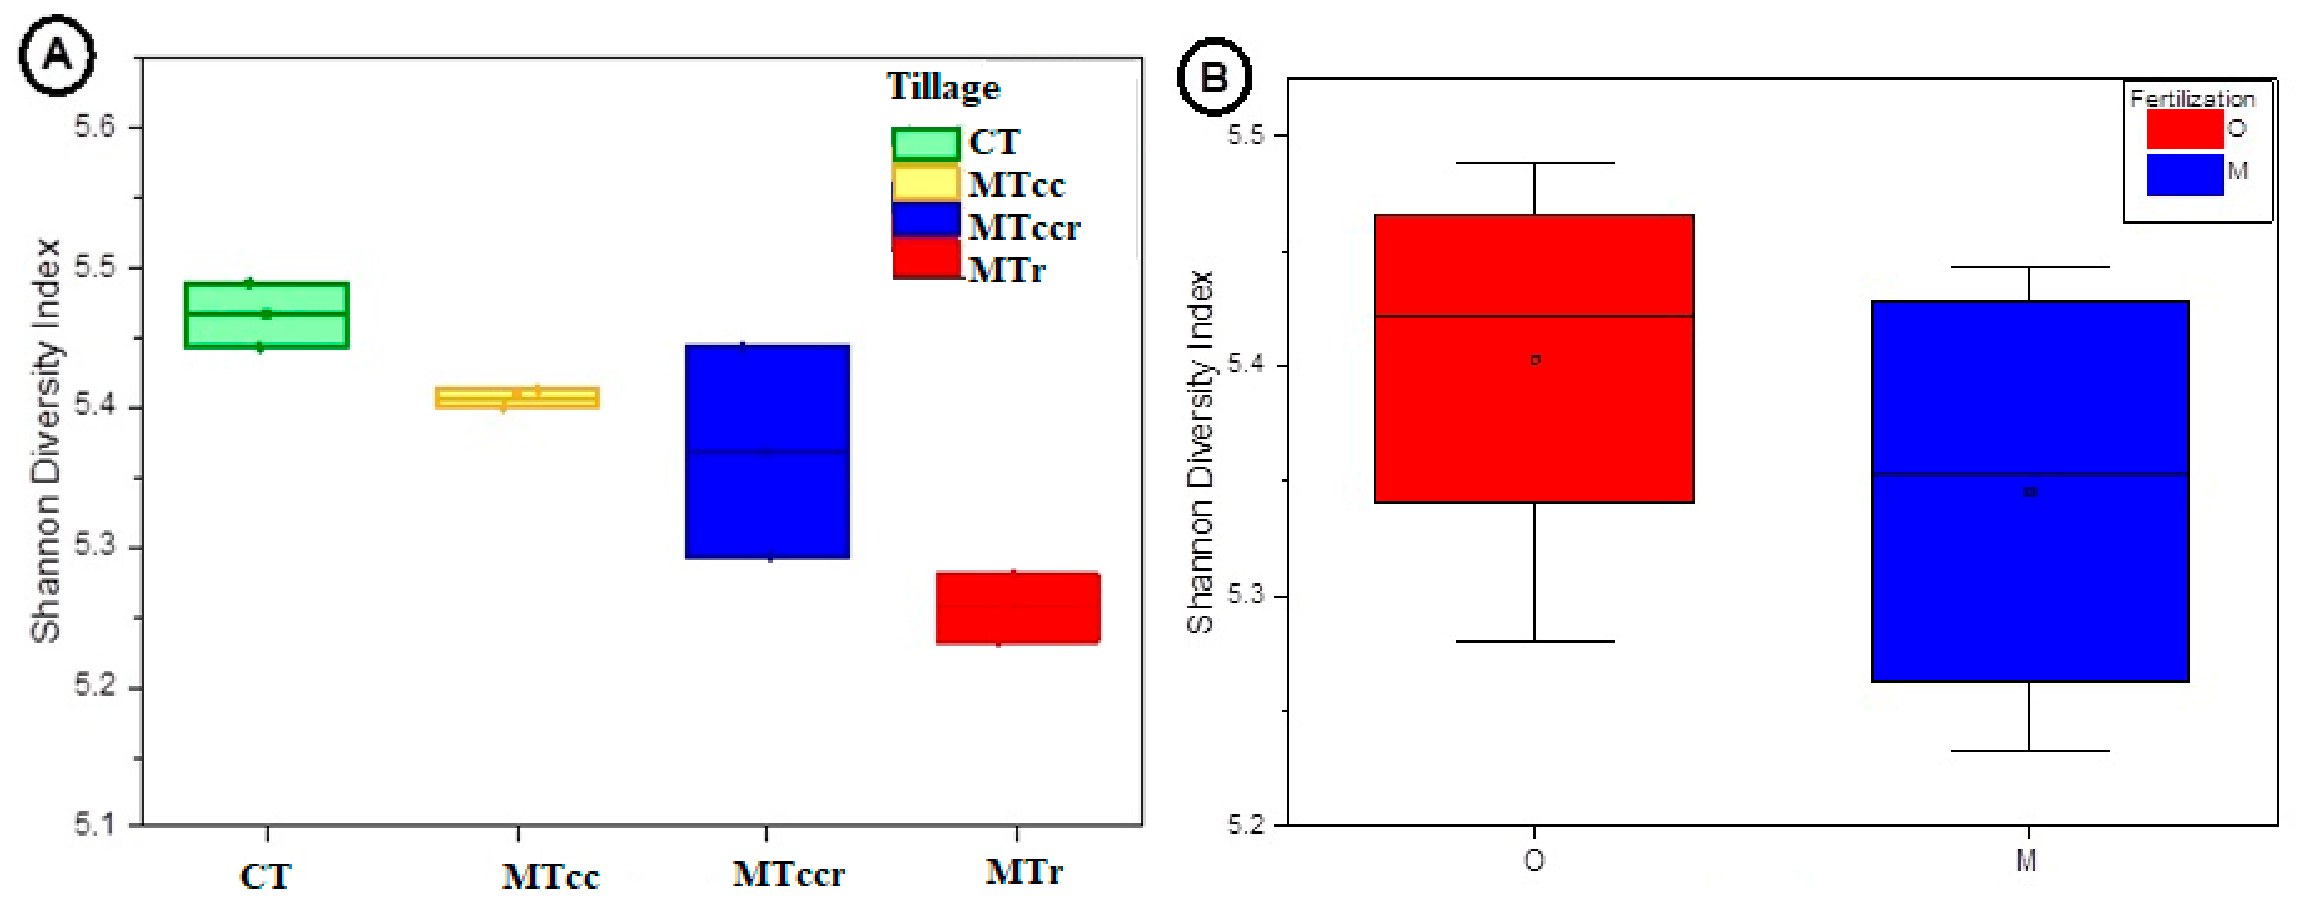
Figure 5 presents the Shannon diversity index values for the soil bacterial populations, according to the experimental factors, namely (A) tillage and (B) fertilization. The Shannon index of the bacterial community was found to vary with the tillage method; in particular, the CT treatment was associated with a higher mean diversity (≈ 5.46 to 5.48), while the MTcc treatment resulted in lower, more homogeneous diversity.
The MTccr treatment using two soil cultivation tools showed greater dispersion, indicating greater variability between the experimental replicates. MTr yielded the lowest values of the Shannon index (≈5.23–5.28)‚ as shown in Figure 6A.
Figure 6.
Shannon diversity index values of bacterial communities according to the two experimental factors: (A) tillage and (B) fertilization. CT: Conventional tillage. CT: Conventional tillage; MTcc: Minimum tillage with cover crop; MTr: Minimum tillage with cultivator; MTccr: Minimum tillage combine cover crop and cultivator.
Figure 6B shows that the diversity index values under the different fertilization methods (O and M) had relatively similar distributions. Although organic fertilization (O) showed a slightly higher median than mineral (M), their interquartile ranges widely overlapped, suggesting that the impact of fertilization on bacterial diversity remains limited compared to that of tillage.
4. Discussion
Several limitations should be considered when interpreting the results of this study. Soil and bacterial changes were only assessed for one growing season, which may not reflect longer-term trends. The experiment was conducted at only one location‚ and the findings may have been influenced by the local soil and other environmental and agricultural factors. The bacterial communities in this study were analyzed via sequencing of 16S rRNA genes and, while this approach provides information on the presence of bacteria at the considered taxonomic level‚ it does not confirm their activity. Other metagenomic and gene-specific techniques could be used to provide further evidence of the mechanisms driving the observed changes in the bacterial communities.
Two other potential weaknesses of this study should be mentioned. The study did not include negative DNA extraction controls‚ and contamination during the DNA extraction process‚ including contamination with other DNA extraction products or other laboratory contaminants‚ may have occurred. Also‚ although the organic fertilizer had been stored and sun-dried for a long time at the study site‚ which was dry‚ this does not guarantee that the organic fertilizer used in this study contained no living microorganisms. Microorganisms introduced in the organic fertilizer may have been part of the soil bacterial populations in this study. Negative DNA extraction controls and other assessments of the bacterial populations in applied organic fertilizers may be useful additions to future studies to control for this source of variation.
As the study lacked an unfertilized control plot for each tillage treatment, the findings related to fertilizer effects should be considered in the context of the specific fertilizer comparisons made in this study. Multi-year studies at multiple locations‚ combined with other molecular techniques and the inclusion of unfertilized controls‚ could help to confirm and extend the results presented in the current study.
It is clear that applying fertilizers has a substantial influence on the amount of OM that builds up in the soil, and that the application of organic (O) fertilizers has a beneficial effect on OM accumulation. It has been shown that organic fertilizers provide soil microorganisms with a substrate on which they can grow and produce soil organic matter [27].
Additionally, the application of mineral fertilizer can also lead to a subsequent increase in soil OM due to an increase in plant biomass, although mineral fertilizers, which mainly contain nitrogen in large quantities, may reduce the OM available for decomposition in the soil [28]; this could explain why the increase in soil OM was greater under organic fertilizers (O) than under mineral fertilizers (M) in the present study.
Recent studies have shown that conservation tillage techniques can help to conserve soil quality and improve its fertility [29]; indeed, low-disturbance tillage techniques have been implemented with the aim of replenishing OC in the topsoil that had been lost due to environmental microbial impoverishment and the resulting oxidation processes [30].
The chickpea is an excellent legume for enriching the soil with nitrogen, which fits perfectly into sustainable farming systems, particularly in the Mediterranean region. As a result of planting this crop, nitrogen levels increased under the various treatments in this study.
This study’s results showed that, although the concentration of each mineral element depends on the tillage technique and fertilizer, it varied depending on the element considered; for example, magnesium (Mg) was the most abundant and least variable mineral element, while phosphorus (P) exhibited the greatest variation. Potassium (K) varied to an intermediate degree, while calcium (Ca) and sodium (Na) were relatively stable.
The variability of phosphorus (P) correlates with the widely accepted idea that, being relatively immobile, P is strongly influenced by OM mineralization, microbial activity, and soil chemical characteristics. Conservation tillage or reduced tillage systems generally promote the accumulation of P in the surface layer, as they disturb the soil less and plant OM is left on the soil surface. Recent analyses, such as those conducted by Lv et al. (2023), have shown that these systems increase the total phosphorus and plant-available phosphorus levels in the surface layers when compared to CT [31].
Potassium (K) did not exhibit as high variability as phosphorus (P), which was likely due to the high potassium content in the soil. However, several studies have shown that no-tillage or reduced tillage practices promote P accumulation in the topsoil due to the retention of residues and avoiding the losses that would otherwise be caused by tillage [32].
The concentrations of Ca and Mg were unaffected and, thus, assumed to be unaltered. However, it has recently been found that conservationist practices increase the concentrations of Ca and Mg in the upper layers of the soil, resulting in an increase in OM due to lower cation exchange capacity and less structural disturbance. In general‚ the effects of agricultural conservation practices tend to be greater after several years of implementation [31].
The least prevalent element was sodium (Na), which remained near zero under all treatments. This observation is in accordance with findings in the literature, which indicate that the effects of tillage on sodium are weak or inconsistent. Available meta-analyses have concluded that no clear trend can be identified regarding the evolution of Na under tillage management systems, in contrast to phosphorus, potassium, calcium, and magnesium [31].
These results confirm that the impacts of the treatments are primarily visible in terms of phosphorus dynamics, while other mineral elements remain relatively stable due to differences in their availability mechanisms. In general, elements whose cycles are strongly linked to biological processes and the decomposition of OM, such as phosphorus, are more sensitive to changes related to soil cultivation.
Meanwhile, cations (i.e., positive ions) such as magnesium and calcium, whose cycles are more dependent on soil mineral reserves, are more stable. The results obtained in this study are in accordance with recent analyses highlighting that reduced-tillage techniques slowly improve the chemical properties, nutrient accumulation, and biological activity in soil [33].
The observed variability in the bacterial community composition is consistent with the impacts of tillage techniques on microbial diversity, including their impacts on bacterial communities due to aggregate fragmentation, accelerated OM mineralization, and changes in air and water circulation conditions in the soil. Conversely, reduced tillage or conservation tillage systems—which leave the soil structure relatively intact—tend to increase OM accumulation and microorganism stability, thus promoting microbial community development.
Most of the tillage systems did not appear to affect the relative ratios between major phyla, suggesting that the taxonomic structure of bacterial communities was relatively stable in this study. Our results show that the bacterial composition is largely dominated by Actinomycetota and Pseudomonadota in tilled soils (CT), which is in technical agreement with the results of the analysis carried out by Wang et al. (2017) [18].
Fertilizer treatments supply soil nutrients and had the greatest main effects on N‚ P‚ and K availability. Other main effects of tillage include changes in other soil characteristics and organic matter decomposition. The greatest main effect of tillage on phosphorus (F= 7.05) may result from biological interactions related to phosphate adsorption by iron and aluminum oxides and mycorrhizal fungi. Significant interactions between tillage and fertilizer treatments for all nutrients (p < 0.05) suggest interactions between tillage and fertilizer treatments that affect nutrient availability. Between tillage and fertilizer treatments for P (F = 8.83) and Mg (F = 7.96), this suggests differences in soil water-holding capacity and other soil characteristics‚ such as pH and rates of nutrient immobilization‚ related to different tillage systems that may limit the effectiveness of fertilizers.
The results obtained in this study revealed that Actinomycetota is the dominant phylum, consistent with several recent studies indicating that this phylum represents one of the most numerous bacterial groups in agricultural soils. These bacteria play indispensable roles in degrading OM, mineralizing nutrients, and retaining soil fertility. As such, a high abundance of these organisms in the microbiome typically correlates with optimal functional capacity, contributing significantly to ensuring the proper functioning of biogeochemical cycles—not only regarding carbon, but also nitrogen [34].
Members of Pseudomonadota, the second most abundant phylum (22–24%), are classified as copiotrophic bacteria that respond promptly to the availability of nutrients and easily degradable organic compounds. As their abundance remained relatively constant among the different treatments, it appears that the tested soil tillage practices did not profoundly change the nutrient resources accessible to this bacterial group. Recent research has also shown that Pseudomonadota actively participate in nutrient transformation processes and the overall functioning of agricultural soils.
Members of the phyla Chloroflexota (12–13%) and Thermoproteota (9–12%) were also present in relatively constant proportions under all treatments. Chloroflexota are often inversely related to the decomposition of more recalcitrant OM compounds and are therefore often favored in soils where OM is relatively stable. Thermoproteota, a phylum of Archaea, seem to be particularly adapted to the oxidation of ammonia—a step in nitrification within the nitrogen cycle. The low level of variation in their abundance between treatments indicates that their associated microbial functions were generally preserved under all conditions.
The minor phyla Bacillota, Gemmatimonadota, Planctomycetota, and Bacteroidota—each comprising less than 5% of the bacterial community—are functionally important for OM recycling, phosphorus and nitrogen cycling, and the resilience of microbial communities to environmental perturbations. The minimal rate of variation among the treatments indicates that there is no significant influence of tillage on microbial communities.
The differences observed between the various treatments were relatively limited; for example, the abundance of Actinomycetota reached 46% under the CT_M treatment. In contrast, this value was 42% under several other treatments. Meanwhile, the abundance of Pseudomonadota varied only between 22 and 24%. These relatively small differences confirm that the tillage method evaluated exerts a moderate influence on the overarching taxonomic composition of each bacterial community in the context of this study; however, this should be interpreted in light of the above-mentioned limitations of this study. Recent studies have indicated that changes brought about by tillage often affect the fine structure of communities, microbial diversity, and interactions between microorganisms, more than the abundances of dominant phyla [35].
Moreover, several studies published between 2023 and 2024 have shown that soil conservation systems—particularly direct seeding or reduced tillage—can influence microbial diversity, bacterial structure stability, and soil functioning, with highly robust variations established in the proportional structure of dominant phyla. Thus, the variations noted in this study agree with the results reported in the recent literature, emphasizing that the effects of tillage are expressed mainly at finer taxonomic levels (genus or species), as well as at the functional level, in microbial communities [36,37].
From the PCA results, it was found that more than two-thirds of the variation in the bacterial community composition can be attributed to the two ecological gradients (tillage practice and fertilizer), which is in agreement with other studies utilizing 16S ribosomal RNA gene profiling data to assess the effects of tillage on the bacterial community structure [38].
In particular, the PC1 axis separated the phyla Pseudomonadota‚ Bacteroidota, and Chloroflexota from Actinomycetota‚ Planctomycetota, and Verrucomicrobiota‚ indicating their differential responses to differences in soil structure. Copiotrophic bacteria such as Pseudomonadota are expected to thrive under conditions characterized by higher carbon and nutrient availability. In contrast‚ soil oligotrophic bacteria such as Actinomycetota utilize high-molecular-weight organic materials as a source of nutrients [39].
The strong positive correlation between Chloroflexota and the PC1 axis is consistent with their roles as decomposers of high-molecular-weight OM and their typical presence in nutrient-poor environments. Planctomycetota and Verrucomicrobiota are mostly found in persistent organic matter-rich soils and soils with complex carbon and nitrogen cycling conditions, which is more likely to be due to differences in ecological factors rather than environmental factors [40].
The second axis primarily varies in Thermoproteota, Nitrospirota, and Euryarchaeota, all of which are strongly involved in nitrogen cycling (e.g., through ammonia oxidation and the various stages of nitrification). Given their strong contribution to the PC2 axis, it is likely that the associated differences between samples are due to differences in nitrogen cycling processes, rather than the taxonomic profile of bacterial communities, according to Wang et al. (2022) [41].
The general proximity of the vectors to the origin in the PCA plot indicates that most of the phyla exhibit relatively small variations. This observation agrees well with a multitude of studies showing that tillage modifies microbial diversity, the relative abundance of specific functional groups, and interactions between microorganisms more than the overall composition of the dominant phyla. Changes induced by cultivation practices are often more pronounced at lower taxonomic levels (e.g., family, genus, or species) than at the phylum level [42].
Despite minor differences in the contributions of a few phyla, the PCA results indicate that bacterial communities generally maintain a stable structure. Long-term experiments comparing various tillage systems often show such stability, with changes mostly affecting microbial roles, their interaction structure, and enzyme activities rather than the dominance of key bacterial phyla. Overall, the PCA results demonstrate significant similarity between several treatments, especially MTr_M, MTcc_M, MTr_O, and MTcc_O, with CT_M appearing as the most differentiated treatment. The results indicate that, although tillage influences the microbial community composition, this impact remains relatively moderate across major bacterial phyla. This observation agrees well with several recent studies showing that tillage modifies the fine structure, interactions, and functions of these microbial communities more than their overall taxonomic composition [35,36,37,38,39,40,41,42,43].
The bacterial community structure had higher F-statistics and lower p-values (less than 0.005) for all phyla than chemical fertilizers did‚ with F-statistic values ranging from 9.01 to 16.12. These findings indicate that soil bacteria may be good early indicators of changes in land management practices. Actinomycetota and Pseudomonadota are copiotrophic bacteria that prefer nutrient-rich conditions and responded strongly to both fertilizer and tillage treatments. Tillage disrupts mycelial mats and increases soil organic matter decomposition‚ favoring r-selected bacteria.
The diversity of microbial communities is widely estimated using the Shannon diversity index, which necessarily takes into account both the relative abundance and taxonomic richness of species at the phylum level. In the current study, Shannon index values between 5.2 and 5.5 were obtained, indicating a high bacterial diversity index characteristic of highly biologically active agricultural soils.
This study’s findings demonstrate that fertilization had a limited impact on bacterial diversity, with tillage acting as the main factor. This result is in accordance with the current understanding that microbial habitats are significantly altered by physical disturbance of the soil, as reported by Navarro-Noya et al. (2013) [42]. Aggregate stability, porosity, oxygen diffusion, water availability, and the vertical distribution of OM are all impacted by tillage activities, and certain bacterial populations are progressively favored over others due to the various ecological conditions created by these changes.
From a soil sustainability perspective‚ findings from this study indicate that multiple soil management strategies are needed. Tillage practices influence soil chemical and biological properties when fertilizer is used. Soil management strategies for different tillage practices can help reduce fertilizer losses and enhance soil biological activity and fertilizer use efficiency.
The highest Shannon values were observed under CT in this study, while MTr (using the cultivator) resulted in the lowest values. This indicates that the various experimental conditions led to very different microbial environments; however, previous studies have established that the effects of tillage on bacterial diversity are not universal. Several studies have shown that minimal or reduced tillage systems can enhance or maintain soil microbial diversity by promoting the preservation of OM and causing less physical disturbance to soil microbial habitats, while other studies have reported decreases in diversity under certain soil and climate conditions. This variability underscores that the ways in which soil bacterial communities react to tillage are highly reliant on the soil type, climate, the duration of experiments, and associated cultivation practices.
5. Conclusions
The present study demonstrated that agricultural tillage methods influence not only the microbial biodiversity of the soil but also its chemical fertility. In particular, phosphorus dynamics and certain aspects of bacterial diversification were impacted. The results revealed that chemical and biological properties of the soil should be integrated simultaneously when evaluating the sustainability of farming systems.
Reduced tillage, using a cover crop in combination with a cultivator and the application of organic fertilizer, increased biodiversity and nutrient levels while eliminating the need for plowing, which degrades agricultural soil. Therefore, this tillage approach is recommended—within this study’s limitations—as the most appropriate farming practice for this type of soil in this region.
The results of this research emphasize the necessity of conservation soil techniques for the preservation of biological quality and fertility in agro-ecological systems. Long-term research, including functional assessments of the microbial community at the phylum level and biological indices, can be expected to deepen our comprehension of the processes that link cropping practices, biogeochemical cycles, and agricultural soil fertility. Such knowledge will allow for the development of agricultural strategies with minimal impacts on microbial biodiversity and maintain soil health, thus being more sustainable while simultaneously optimizing productivity.
Supplementary Materials
The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/agrochemicals5040052/s1, Table S1: Taxonomy.
Author Contributions
Conceptualization, A.K., A.H. and M.L.; methodology, A.K., A.H. and M.L.; software, A.K.; validation, A.K. and A.H.; formal analysis, A.K. and A.S.; investigation, A.K.; resources, A.K., A.H. and M.L.; data curation, A.K. and A.H.; writing—original draft preparation, A.K., A.H. and M.L.; writing—review and editing, A.K., A.H., M.L. and A.S.; visualization, A.K., A.H., M.L. and A.S.; supervision, A.K. and A.S. All authors have read and agreed to the published version of the manuscript.
Funding
This research received no external funding. All analyses were performed on our own behalf.
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
The corresponding author can provide the data used in this study upon reasonable request. The 16S rRNA gene sequencing data generated in this study have been deposited in the NCBI Sequence Read Archive (SRA) under BioProject accession number PRJNA1551531.
Acknowledgments
I thanks Lahcen BOUDIA, state engineer in agronomy, for helping me to carry out the chemical analysis of the soil at the FERTIAL Company in Oran, Algeria. I would also like to thank Abdelhafid SEBIHI for encouraging and supporting me in the writing of my doctoral thesis.
Conflicts of Interest
The authors declare no conflicts of interest.
Abbreviations
The following abbreviations are used in this manuscript:
| ANOVA | Analysis of variance |
| CT | Conventional tillage |
| MT | Minimum tillage |
| MTcc | Minimum tillage with cover crop |
| MTr | Minimum tillage with cultivator |
| MTccr | Minimum tillage with cover crop and cultivator |
| M | Mineral fertilizer |
| O | Organic fertilizer |
| OC | Organic carbon |
| OM | Organic matter |
| PCA | Principal Components Analysis |
| RCBD | Randomized complete block design |
References
- Pradhan, N.; Singh, S.; Saxena, G.; Pradhan, N.; Koul, M.; Kharkwal, A.C.; Sayyed, R. A Review on Microbe–Mineral Transformations and Their Impact on Plant Growth. Front. Microbiol. 2025, 16, 1549022. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dai, Z.; Guo, X.; Lin, J.; Wang, X.; He, D.; Zeng, R.; Meng, J.; Luo, J.; Delgado-Baquerizo, M.; Moreno-Jiménez, E.; et al. Metallic Micronutrients Are Associated with the Structure and Function of the Soil Microbiome. Nat. Commun. 2023, 14, 8456. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wilhelm, R.C.; Amsili, J.P.; Kurtz, K.S.M.; Van Es, H.M.; Buckley, D.H. Ecological Insights into Soil Health According to the Genomic Traits and Environment-Wide Associations of Bacteria in Agricultural Soils. ISME Commun. 2023, 3, 1. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wongkiew, S.; Chaikaew, P.; Takrattanasaran, N.; Khamkajorn, T. Evaluation of Nutrient Characteristics and Bacterial Community in Agricultural Soil Groups for Sustainable Land Management. Sci. Rep. 2022, 12, 7368. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jacoby, R.; Peukert, M.; Succurro, A.; Koprivova, A.; Kopriva, S. The Role of Soil Microorganisms in Plant Mineral Nutrition—Current Knowledge and Future Directions. Front. Plant Sci. 2017, 8, 1617. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lowenfels, J.; Lewis, W. Teaming with Microbes: A Gardener’s Guide to the Soil Food Web; Timber Press: Portland, OR, USA, 2006. [Google Scholar]
- Hayat, R.; Ali, S.; Amara, U.; Khalid, R.; Ahmed, I. Soil Beneficial Bacteria and Their Role in Plant Growth Promotion: A Review. Ann. Microbiol. 2010, 60, 579–598. [Google Scholar] [CrossRef] [Scilit]
- Insam, H.; Klammsteiner, T.; Gómez-Brandòn, M. Biology of Compost. In Encyclopedia of Soils in the Environment; Elsevier: Amsterdam, The Netherlands, 2023; pp. 522–532. [Google Scholar] [CrossRef] [Scilit]
- Wahab, A.; Bibi, H.; Batool, F.; Muhammad, M.; Ullah, S.; Zaman, W.; Abdi, G. Plant Growth-Promoting Rhizobacteria Biochemical Pathways and Their Environmental Impact: A Review of Sustainable Farming Practices. Plant Growth Regul. 2024, 104, 637–662. [Google Scholar] [CrossRef] [Scilit]
- Ribeiro, I.D.A.; Volpiano, C.G.; Vargas, L.K.; Granada, C.E.; Lisboa, B.B.; Passaglia, L.M.P. Use of Mineral Weathering Bacteria to Enhance Nutrient Availability in Crops: A Review. Front. Plant Sci. 2020, 11, 590774. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Uroz, S.; Oger, P.; Lepleux, C.; Collignon, C.; Frey-Klett, P.; Turpault, M.-P. Bacterial Weathering and Its Contribution to Nutrient Cycling in Temperate Forest Ecosystems. Res. Microbiol. 2011, 162, 820–831. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Okorie, B.O.; Niraj, Y. Effects of Different Tillage Practices on Soil Fertility Properties: A Review. Int. J. Agric. Environ. Res. 2022, 8, 176–193. [Google Scholar] [CrossRef]
- Hartman, M.; Six, J. Soil Structure and Microbiome Functions in Agro ecosystems. Nat. Rev. Earth Environ. 2022, 4, 4–18. [Google Scholar] [CrossRef] [Scilit]
- Husnjak, S.; Filipović, D.; Košutić, S. Influence of Different Tillage Systems on Soil Physical Properties and Crop Yield. Plant Soil Environ. 2002, 48, 249–254. [Google Scholar] [CrossRef] [Scilit]
- Bezboruah, M.; Sharma, S.K.; Laxman, T.; Ramesh, S.; Sampathkumar, T.; Gulaiya, S.; Malathi, G.; Krishnaveni, S.A. Conservation Tillage Practices and Their Role in Sustainable Farming Systems. J. Exp. Agric. Int. 2024, 46, 946–959. [Google Scholar] [CrossRef] [Scilit]
- Diop, M.; Beniaich, A.; Cicek, H.; Ouabbou, H.; El Gharras, O.; Tanji, A.; Bamouh, A.; Dahan, R.; Zine El Abidine, A.; El Gharous, M.; et al. Effects of Occasional Tillage on Soil Physical and Chemical Properties and Weed Infestation in a 10-Year No-till System. Front. Environ. Sci. 2024, 12, 1431822. [Google Scholar] [CrossRef] [Scilit]
- Yuan, C.; Ma, Z.; Liu, S.; Nie, H.; Feng, G.; Wang, S.; Luo, S. Effects of Strip Tillage on Soil Microbial Community’ Structure and Function in Black Soil. Front. Microbiol. 2025, 16, 1730920. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, Z.; Liu, L.; Chen, Q.; Wen, X.; Liu, Y.; Han, J.; Liao, Y. Conservation Tillage Enhances the Stability of the Rhizosphere Bacterial Community Responding to Plant Growth. Agron. Sustain. Dev. 2017, 37, 44. [Google Scholar] [CrossRef] [Scilit]
- Gupta, A.; Singh, U.B.; Sahu, P.K.; Paul, S.; Kumar, A.; Malviya, D.; Singh, S.; Kuppusamy, P.; Singh, P.; Paul, D.; et al. Linking Soil Microbial Diversity to Modern Agriculture Practices: A Review. Int. J. Environ. Res. Public Health 2022, 19, 3141. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ziane, A.; Douaoui, A.; Yahiaoui, I.; Pulido, M.; Larid, M.; Gulakhmadov, A.; Chen, X. ‘Upgrading the Salinity Index Estimation and Mapping Quality of Soil Salinity Using Artificial Neural Networks in the Lower-Cheliff Plain of Algeria in North Africa’: Amélioration de l’estimation de l’indice de Salinité et de La Qualité de La Cartographie de La Salinité Des Sols En Utilisant Les Réseaux de Neurones Artificiels Dans La Plaine Du Bas Cheliff Au Nord de l’Algérie. Can. J. Remote Sens. 2022, 48, 182–196. [Google Scholar] [CrossRef] [Scilit]
- Yu, Y.; Flury, M. How to Take Representative Samples to Quantify Microplastic Particles in Soil? Sci. Total Environ. 2021, 784, 147166. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Roper, W.R.; Robarge, W.P.; Osmond, D.L.; Heitman, J.L. Comparing Four Methods of Measuring Soil Organic Matter in North Carolina Soils. Soil Sci. Soc. Am. J. 2019, 83, 466–474. [Google Scholar] [CrossRef] [Scilit]
- Lewis, W.H.; Tahon, G.; Geesink, P.; Sousa, D.Z.; Ettema, T.J.G. Innovations to Culturing the Uncultured Microbial Majority. Nat. Rev. Microbiol. 2021, 19, 225–240. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hong Nhien, H.T.T.; Nguyen, G.T. Evaluation of Surface Water Quality Using Biodiversity Indices in Phu My Species-Habitat Conservation Area, Kien Giang Province, Vietnam. Ecol. Eng. Environ. Technol. 2024, 25, 102–112. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bolyen, E.; Rideout, J.R.; Dillon, M.R.; Bokulich, N.A.; Abnet, C.C.; Al-Ghalith, G.A.; Alexander, H.; Alm, E.J.; Arumugam, M.; Asnicar, F.; et al. Reproducible, Interactive, Scalable and Extensible Microbiome Data Science Using QIIME 2. Nat. Biotechnol. 2019, 37, 852–857. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Quast, C.; Pruesse, E.; Yilmaz, P.; Gerken, J.; Schweer, T.; Yarza, P.; Peplies, J.; Glöckner, F.O. The SILVA Ribosomal RNA Gene Database Project: Improved Data Processing and Web-Based Tools. Nucleic Acids Res. 2012, 41, D590–D596. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wan, Q.; Zhu, G.; Guo, H.; Zhang, Y.; Pan, H.; Yong, L.; Ma, H. Influence of Vegetation Coverage and Climate Environment on Soil Organic Carbon in the Qilian Mountains. Sci. Rep. 2019, 9, 17623. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Moeskops, B.; Buchan, D.; Van Beneden, S.; Fievez, V.; Sleutel, S.; Gasper, M.S.; D’Hose, T.; De Neve, S. The Impact of Exogenous Organic Matter on SOM Contents and Microbial Soil Quality. Pedobiologia 2012, 55, 175–184. [Google Scholar] [CrossRef] [Scilit]
- Radicetti, E.; Osipitan, O.A.; Langeroodi, A.R.S.; Marinari, S.; Mancinelli, R. CO2 Flux and C Balance Due to the Replacement of Bare Soil with Agro-Ecological Service Crops in Mediterranean Environment. Agriculture 2019, 9, 71. [Google Scholar] [CrossRef] [Scilit]
- Radicetti, E.; Campiglia, E.; Langeroodi, A.S.; Zsembeli, J.; Mendler-Drienyovszki, N.; Mancinelli, R. Soil Carbon Dioxide Emissions in Eggplants Based on Cover Crop Residue Management. Nutr. Cycl. Agroecosyst. 2020, 118, 39–55. [Google Scholar] [CrossRef] [Scilit]
- Lv, L.; Gao, Z.; Liao, K.; Zhu, Q.; Zhu, J. Impact of Conservation Tillage on the Distribution of Soil Nutrients with Depth. Soil Tillage Res. 2023, 225, 105527. [Google Scholar] [CrossRef] [Scilit]
- Nunes, M.R.; Karlen, D.L.; Moorman, T.B.; Cambardella, C.A. How Does Tillage Intensity Affect Chemical Soil Health Indicators? A United States Meta-analysis. Agrosystems Geosci. Environ. 2020, 3, e20083. [Google Scholar] [CrossRef] [Scilit]
- Wen, L.; Peng, Y.; Lin, Y.; Zhou, Y.; Cai, G.; Li, B.; Chen, B. Conservation Tillage Increases Nutrient Accumulation by Promoting Soil Enzyme Activity: A Meta-Analysis. Plant Soil 2025, 508, 531–546. [Google Scholar] [CrossRef] [Scilit]
- Philippot, L.; Chenu, C.; Kappler, A.; Rillig, M.C.; Fierer, N. The Interplay between Microbial Communities and Soil Properties. Nat. Rev. Microbiol. 2024, 22, 226–239. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Khan, N.; Humm, E.A.; Jayakarunakaran, A.; Hirsch, A.M. Reviewing and Renewing the Use of Beneficial Root and Soil Bacteria for Plant Growth and Sustainability in Nutrient-Poor, Arid Soils. Front. Plant Sci. 2023, 14, 1147535. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ibáñez, A.; Sombrero, A.; Santiago-Pajón, A.; Santiago-Calvo, Y.; Asensio-S.-Manzanera, M.C. Effect of Long-Term Conservation Tillage Management on Microbial Diversity under Mediterranean Rainfed Conditions. Soil Tillage Res. 2024, 236, 105923. [Google Scholar] [CrossRef] [Scilit]
- Zhu, Y.; Zhang, H.; Wang, Q.; Zhu, W.; Kang, Y. Soil Extracellular Enzyme Activity Linkage with Soil Organic Carbon under Conservation Tillage: A Global Meta-Analysis. Eur. J. Agron. 2024, 155, 127135. [Google Scholar] [CrossRef] [Scilit]
- Dong, F.; Wang, L.; Xu, T.; Yan, Q.; Yan, S.; Li, F.; Chen, L.; Zhang, R. Multi-Omics Analysis of Soil Microbiota and Metabolites in Dryland Wheat Fields under Different Tillage Methods. Sci. Rep. 2024, 14, 24066. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, C.; Li, L.; Xie, J.; Coulter, J.A.; Zhang, R.; Luo, Z.; Cai, L.; Wang, L.; Gopalakrishnan, S. Soil Bacterial Diversity and Potential Functions Are Regulated by Long-Term Conservation Tillage and Straw Mulching. Microorganisms 2020, 8, 836. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Górska, E.B.; Stępień, W.; Hewelke, E.; Lata, J.-C.; Gworek, B.; Gozdowski, D.; Sas-Paszt, L.; Bazot, S.; Lisek, A.; Gradowski, M.; et al. Response of Soil Microbiota to Various Soil Management Practices in 100-Year-Old Agriculture Field and Identification of Potential Bacterial Ecological Indicator. Ecol. Indic. 2024, 158, 111545. [Google Scholar] [CrossRef] [Scilit]
- Wang, Y.; Chen, G.; Sun, Y.; Zhu, K.; Jin, Y.; Li, B.; Wang, G. Different Agricultural Practices Specify Bacterial Community Compositions in the Soil Rhizosphere and Root Zone. Soil Ecol. Lett. 2022, 4, 18–31. [Google Scholar] [CrossRef] [Scilit]
- Navarro-Noya, Y.E.; Gómez-Acata, S.; Montoya-Ciriaco, N.; Rojas-Valdez, A.; Suárez-Arriaga, M.C.; Valenzuela-Encinas, C.; Jiménez-Bueno, N.; Verhulst, N.; Govaerts, B.; Dendooven, L. Relative Impacts of Tillage, Residue Management and Crop-Rotation on Soil Bacterial Communities in a Semi-Arid Agro ecosystem. Soil Biol. Biochem. 2013, 65, 86–95. [Google Scholar] [CrossRef] [Scilit]
- Cao, X.; Liu, J.; Zhang, L.; Mao, W.; Li, M.; Wang, H.; Sun, W. Response of Soil Microbial Ecological Functions and Biological Characteristics to Organic Fertilizer Combined with Biochar in Dry Direct-Seeded Paddy Fields. Sci. Total Environ. 2024, 948, 174844. [Google Scholar] [CrossRef] [Scilit] [PubMed]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.