


Abstract
Virtual reality (VR) has emerged as a powerful tool in neuroscience and psychiatry, providing immersive and ecologically valid environments to investigate human cognition. Stress is known to disrupt core cognitive functions, particularly learning and memory, which are critical for mental health. While classical paradigms such as the radial arm maze have yielded fundamental insights into animal research, their application in humans has been limited. The aim of this study was to develop NeuroHM, a VR-based radial arm maze, to evaluate spatial learning and memory in adults under experimentally induced stress. A total of 100 participants were recruited and randomly assigned to either a control group (n = 50) or a stress group (n = 50). Participants navigated the virtual radial arm maze from a first-person perspective, relying on distal planetary landmarks to maintain spatial orientation and recall spatial locations. The primary dependent variables were working memory errors, reference memory errors, and latency. Salivary cortisol levels were collected to validate the stress induction protocol and to examine the relationship between stress and cognitive performance. Participants in the stress group showed increased latency and higher reference memory errors compared to controls, with working memory exhibiting the most pronounced impairment. Our findings show that acute stress significantly disrupts cognition and highlight NeuroHM as a promising tool for cognitive assessment in mental health research.
1. Introduction
Stress has been one of the most extensively investigated adaptive responses. It is defined as an organism’s reaction to perceived demands or threats that challenge internal stability [1]. Exposure to stressors activates the autonomic and neuroendocrine systems to restore homeostasis. Physiologically, this involves stimulation of both the sympatho-adreno-medullary (SAM) system and the hypothalamic–pituitary–adrenal (HPA) axis [2,3]. Activation of the SAM system triggers the release of catecholamines such as adrenaline and noradrenaline, resulting in increased heart rate and blood pressure. In parallel, activation of the HPA axis promotes the secretion of glucocorticoids such as cortisol into the bloodstream. Cortisol exerts a profound influence on brain function, and the hippocampus is particularly sensitive to its effects [4,5]. Neurobehavioral research has consistently shown that stress-related hippocampal dysfunction disrupts spatial learning and memory processes in mammals [6,7,8], including humans [9,10,11,12]. Parallel research demonstrates that acute stress selectively disrupts hippocampal-based navigation and biases behavior toward caudate-dependent response strategies [13,14,15].
Spatial learning and memory are fundamental cognitive functions that allow individuals to encode, store, and retrieve information about environmental layout and spatial orientation [16]. Numerous experimental paradigms have been developed to assess these abilities under stress conditions. Among the most frequently used protocols in humans are psychological stressors such as time-pressured arithmetic, the Stroop task, or complex problem-solving matrices, which reliably engage stress responsive systems and have become standard tools for acute stress induction in laboratory settings [17,18,19,20].
In pre-clinical research, the radial arm maze (RAM) or Morris Water Maze (MWM) are the most established paradigms for assessing spatial learning and memory in rodents [21,22]. In this task, animals must learn to retrieve rewards from specific maze arms while avoiding repeated entries into non-rewarded ones. The mazes provide quantitative measures of reference memory, which reflects long-term learning of rewarded locations, and working memory, which reflects short-term updating of recently visited locations [21,22]. However, adapting the RAM to human testing presents significant logistical and methodological limitations. A physical human-scale maze would require considerable space; most human studies therefore rely on paper and pencil tasks. These traditional neuropsychological assessments often lack ecological validity because they require participants to imagine spatial transformations or manipulate visual objects in abstract contexts rather than navigate real or realistic environments.
Given these constraints, there is a growing need for experimental tools that can more directly assess hippocampal-dependent spatial learning and memory. Tasks involving spatial navigation and temporal sequencing of events provide a more comprehensive and sensitive measure of episodic memory than conventional verbal or object recognition tests [23]. The recent advancement of VR technology provides an unprecedented opportunity to meet these methodological needs [24]. VR enables the creation of immersive and interactive environments that combine high ecological validity with precise experimental control [25]. Virtual environments can be designed to simulate an almost infinite range of conditions while maintaining cost-effectiveness and experimental precision [26]. This approach allows the assessment of behaviors that would be difficult or impossible to reproduce in traditional laboratory settings, such as large-scale navigation or dynamic spatial problem solving.
Although RAM paradigms have traditionally been applied in rodents, several human studies have adapted RAM-like or large-scale navigation tasks into virtual environments. Spieker et al. [27], for example, implemented the virtual radial arm maze (VRAM) in adults and demonstrated that this paradigm is sensitive to spatial memory deficits associated with prefrontal and hippocampal dysfunction in schizophrenia, supporting its translational value for bridging clinical practice and research. More recently, Palombi et al. [24,28] reviewed the application of both real-world and VRAM tasks in humans, emphasizing their utility for dissociating working memory from reference memory processes and for evaluating spatial abilities in controlled yet ecologically relevant settings. The use of VR-based navigation tasks has also expanded in clinical and aging populations, as indicated by a recent systematic review showing growing adoption of virtual reality and serious-game-based instruments for assessing spatial navigation and memory in individuals at risk of Alzheimer’s disease and related disorders [29]. Complementing this evidence, studies such as Laczó et al. [30] have shown that VR-based radial or multi-arm mazes are sensitive to subtle hippocampal impairments in individuals with genetic or clinical risk of cognitive decline. Collectively, these findings support the potential of immersive VR-maze paradigms to capture hippocampal-dependent spatial learning strategies in humans.
Conventional neuropsychological assessments remain widely used in clinical contexts for identifying cognitive decline. However, their diagnostic sensitivity can be reduced by confounding variables such as education, age, examiner expertise, and testing environment. In contrast, VR-based paradigms can minimize these confounds by standardizing the testing context and engaging participants in realistic and embodied cognitive experiences [31]. Despite the increasing interest in immersive cognitive assessment, evidence is still scarce regarding the use of spatial memory performance as a discriminative marker for different mental health conditions [32,33,34].
In the present study, we developed an immersive virtual reality adaptation of the radial eight-arm maze named NeuroHM, designed to evaluate spatial learning and memory under controlled experimental conditions. The primary objective of this pilot study was to examine how experimentally induced acute stress affects spatial learning and memory in adults and to evaluate the feasibility of NeuroHM as a reliable tool for detecting early cognitive alterations related to stress and mental health conditions.
2. Materials and Methods
All procedures were approved by the Ethical Committees of CUCS UdeG (CUCS/CINV/0017/25) University’s Ethics Committee in accordance with the Declaration of Helsinki. Prior to testing, subjects were briefed on the study’s aims and required to sign informed consent forms. All participants provided their consent. No participants reported being prescribed any psychiatric medications.
2.1. Participants
A demographic questionnaire was used to assess age, sex, education level, and prescribed medication situation (Table 1). One hundred participants were recruited through advertisements posted on the Universidad de Guadalajara, Centro Universitario de Ciencias de la Salud (CUCS) campus. Male and female volunteers were randomly assigned to either the control group (n = 50) or the stress group (n = 50), ensuring an equal distribution between conditions. To control baseline cognitive ability, all participants confirmed having no history of learning difficulties and reported normal academic functioning. No individual had prior experience with virtual radial maze tasks or similar spatial navigation paradigms.
Table 1.
Demographic summary of the 100 participants included in the study.
2.2. Inclusion/Exclusion Criteria
Potential participants were screened according to predefined exclusion criteria. Individuals were excluded if they presented (1) physical impairments that could interfere with task performance, (2) a diagnosis or history of major neurocognitive disorders or psychiatric conditions as defined by the DSM-5, including schizophrenia spectrum disorders, mood disorders, anxiety disorders, or developmental conditions, or (3) a history of alcohol abuse or current use of illicit substances. Inclusion criteria specified that participants had to be between 18 and 35 years of age, demonstrate normal or corrected-to-normal visual acuity (20/20), and possess the ability to complete a demographic questionnaire and accurately follow the instructions required for the allocentric navigation task.
2.3. Sample Size
Recruitment took place from May to August 2025 with a targeted sample size of ≥50 per group. This sample size was chosen to ensure adequate statistical power for our comparisons. Power analysis was conducted using GPower (v3.1.). Based on a Generalized linear model using within- and between-subjects interaction and a power of β = 0.80, a significance level of α = 0.05, and a medium effect size of f = 0.25, a total of 90 participants were needed. To ensure robust group balance, allow for attrition, and align with feasibility constraints typical of pilot-stage VR studies, the target sample was set at 100 participants.
This sample size is consistent with precedent in the virtual-reality and cognitive-assessment literature. For example, Shen et al. [35] evaluated the usability and psychometric validity of a VR-based cognitive assessment (VR-CAT) in 54 participants, supporting the adequacy of moderate samples in early-phase validation contexts. Similarly, Jespersen et al. [36] outlined a randomized VR cognitive remediation trial with 66 patients, reflecting common sample sizes in VR-based cognitive clinical protocols. Further, an exploratory randomized controlled trial by Garrett et al. [37] assessing VR as a non-pharmacological intervention for chronic pain included 110 adults (≈55 participants per arm), demonstrating that group sizes in the range of 25–60 participants are typical in early-stage or feasibility VR trials.
The representativeness of our sample is limited to a healthy young-adult university population. Although age and sex distributions were balanced across groups due to random assignment, the demographic homogeneity may constrain generalizability.
2.4. Equipment and Software
The experiment was developed and executed using the Unity game engine on a desktop PC with an Intel i7-12650H, 2300 Mhz CPU (MSI Cyborg 15 A12V), RAM 64 GB, and Nvidia RTX 4050 GPU. Immersive presentation of the virtual environment was delivered through the Meta Quest 3S visor (model P97), a standalone virtual reality headset featuring high-resolution displays, inside-out tracking with integrated cameras, a 110° field of view, and ergonomic hand-held controllers that enable precise interaction with three-dimensional environments.
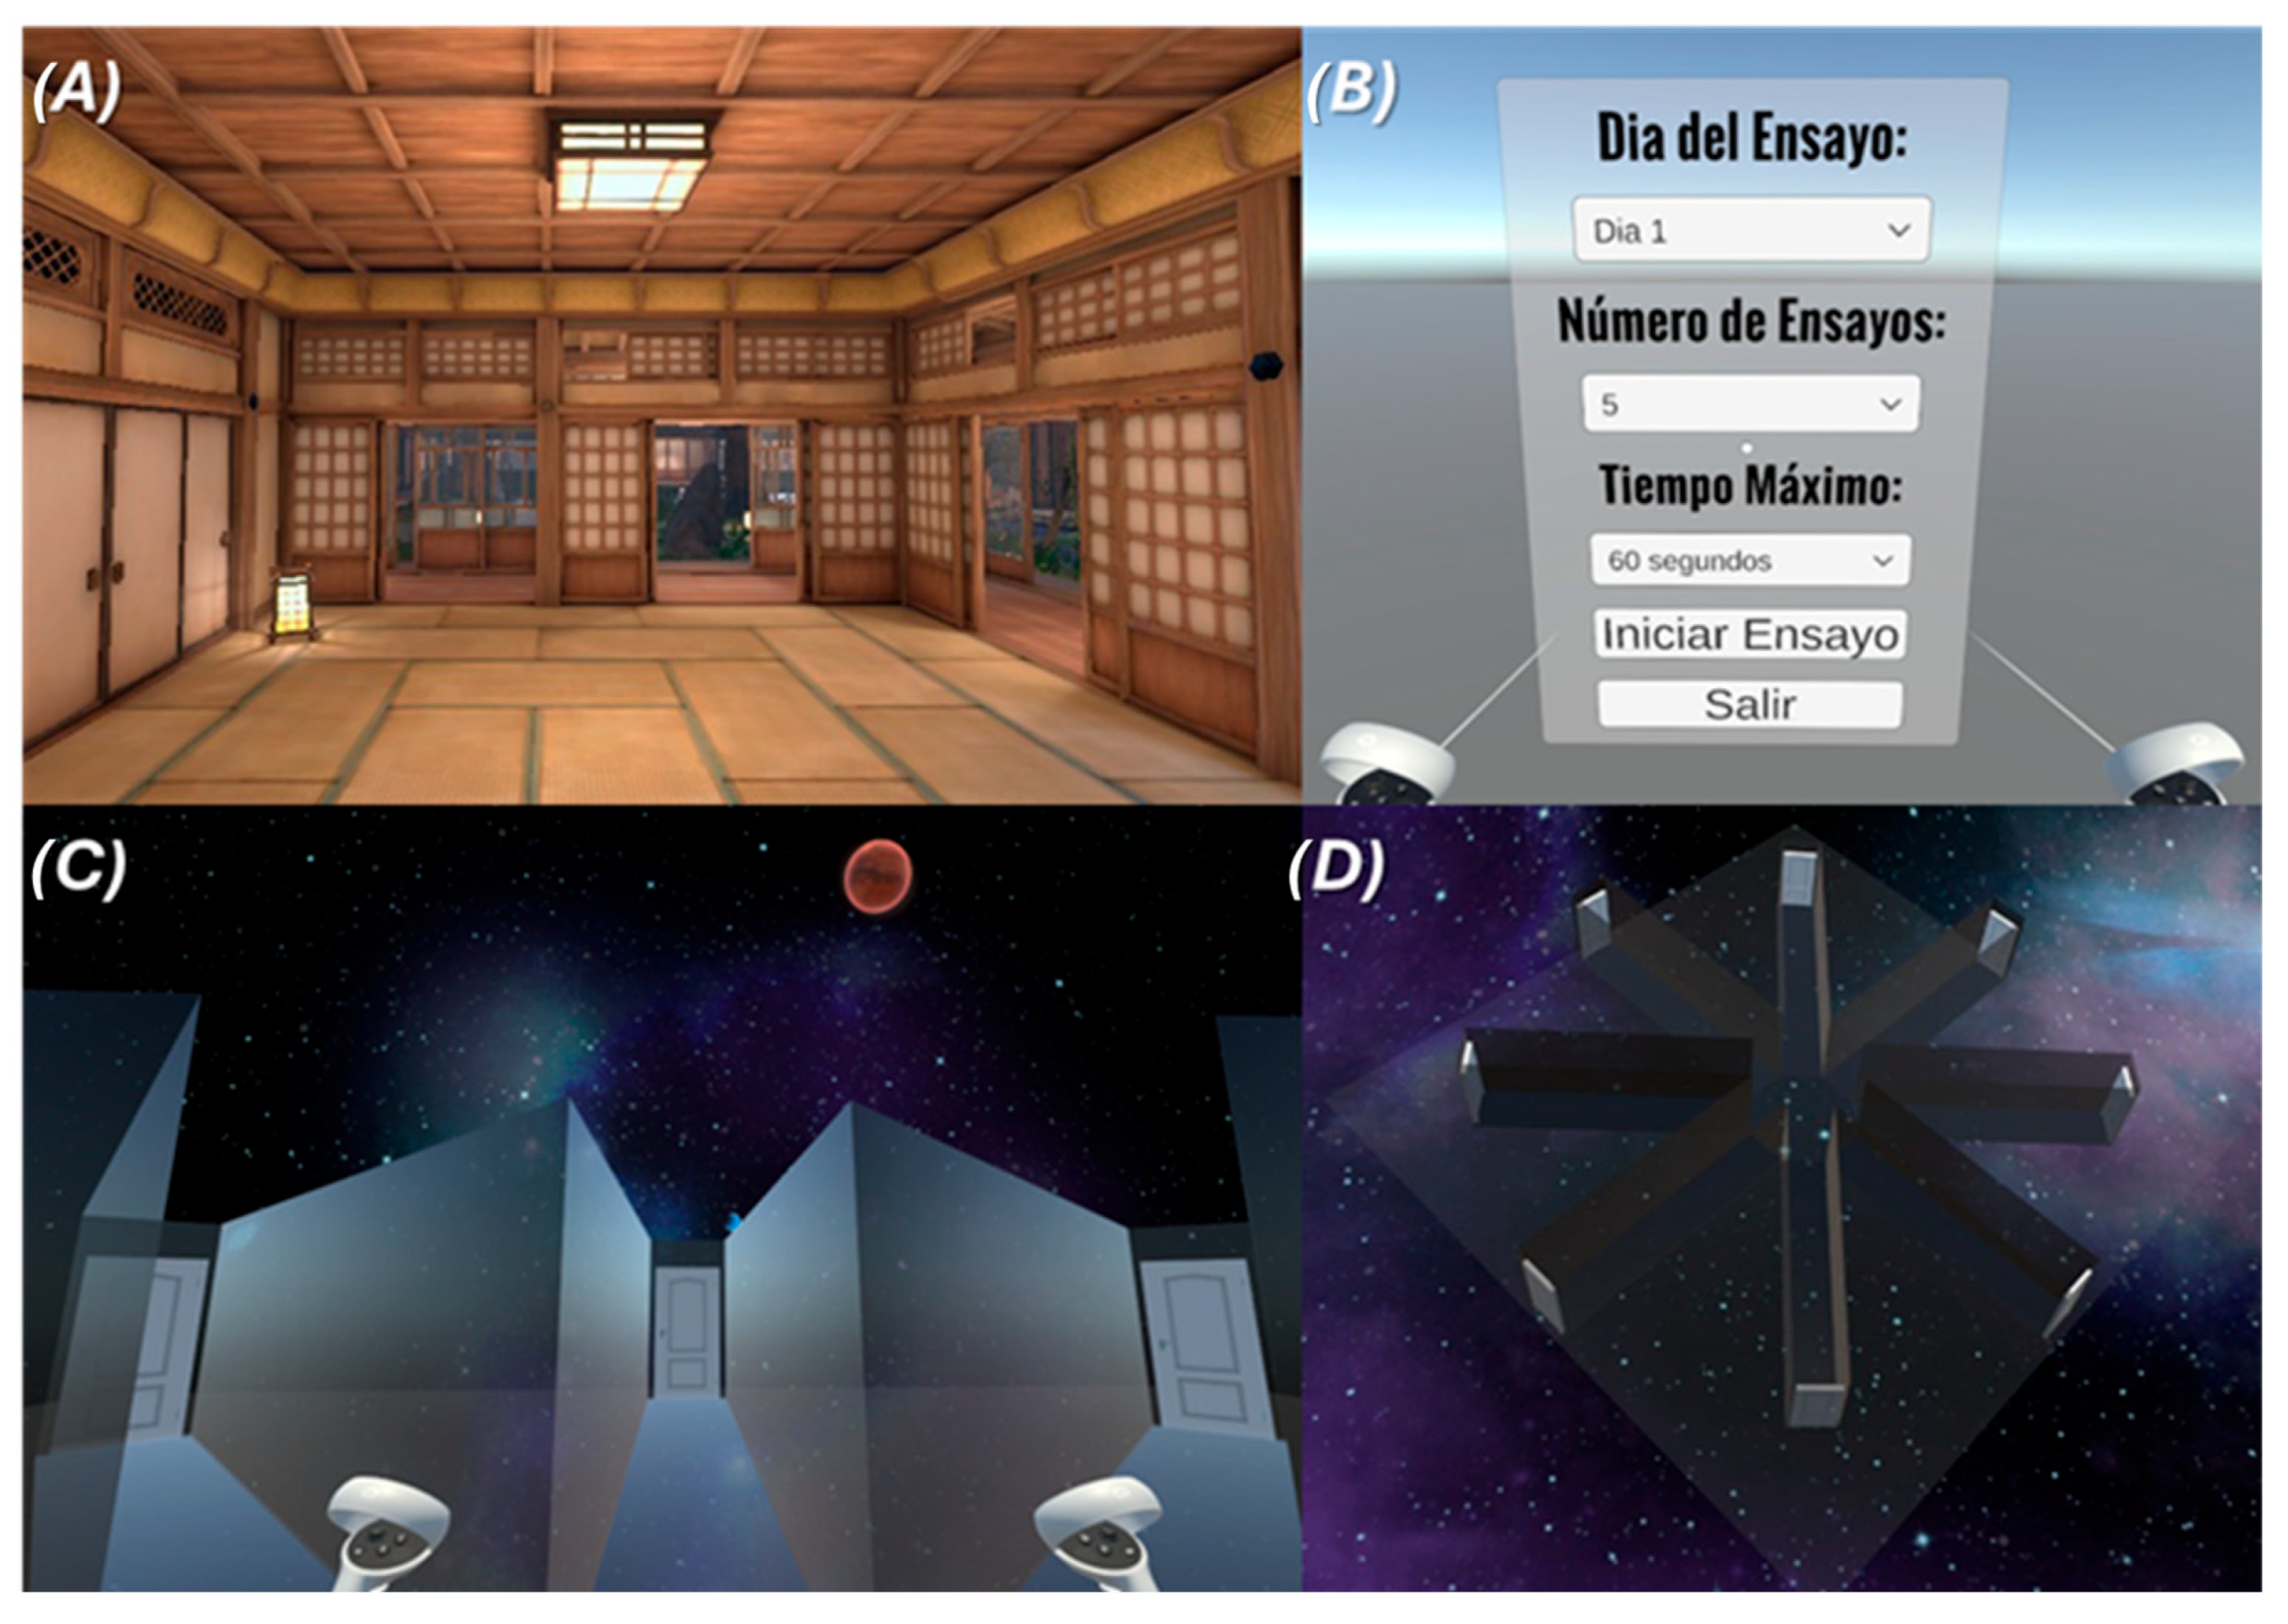
We created a Virtual Radial Eight-Arm Maze program (NeuroHM) using a Unity game engine (Unity Technologies, San Francisco, CA, USA version 6000.1.0f1). The virtual environment was constructed in three dimensions with a central octagonal platform (width: 6 m × length: 6 m) from which eight immersive equidistant arms (width: 2 m × length: 12 m × height: 4 m) extended radially (Figure 1). Each arm was designed with a uniform width and length, bounded by walls to prevent participants from leaving the defined pathway. All arms of the maze ended in visible doors, with four exit doors fixed in place. To provide distal spatial cues for allocentric navigation, four large planetary objects were positioned at the cardinal points around the maze. Participants could observe their environment at 360° by turning their heads and bodies while using the virtual reality Meta Quest 3S visor; direction of movement was determined using a hand-held controller.
Figure 1.
NeuroHM. (A) Virtual waiting room used between trials, where participants in the control group were allowed to move freely. (B) Main menu interface for configuring experimental parameters, including session day, number of trials, and maximum time allowed. (C) First-person perspective within the maze, showing doors at the end of arms and distal spatial cues such as planetary objects and galactic textures for allocentric navigation. (D) Overhead view of the radial eight-arm maze layout, illustrating the spatial arrangement of arms with exit and closed pathways.
2.5. Experimental Design
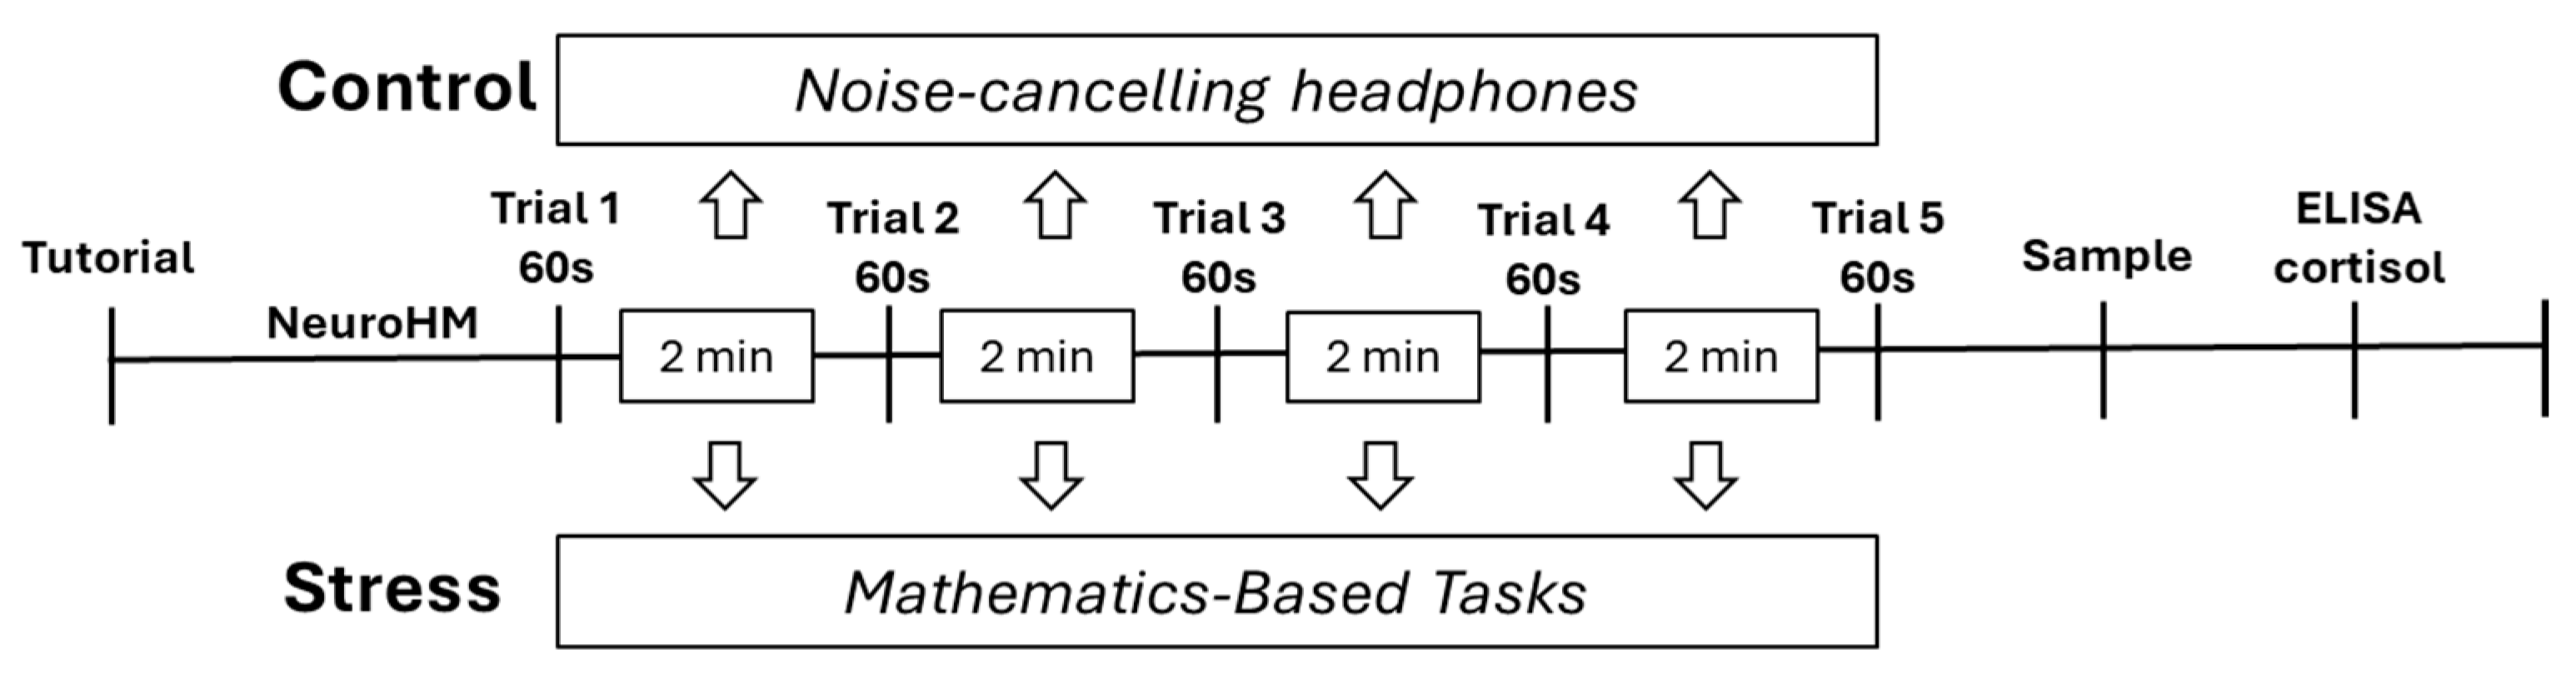
Participants were randomly assigned to either the control or the stress condition. The control group was not exposed to additional stimuli and remained in a quiet environment using noise-cancelling headphones throughout the session. In contrast, the stress group underwent cognitive stress induction during each two-minute intertrial interval (Figure 2).
Figure 2.
Schematic representation of the experimental timeline.
2.6. Stress Induction Procedure
Participants were randomly assigned to either the acute stress or control condition using Study Randomizer (Study Randomizer Available from: https://www.studyrandomizer.com, accessed on 18 August 2025), a web-based randomization tool designed for experimental research. The software generated a concealed 1:1 allocation sequence using permuted block randomization to ensure balanced group distribution throughout recruitment. The allocation list was not accessible to the experimenters administering the VR task, thus maintaining allocation concealment and reducing potential bias.
Acute stress was induced through a high-load cognitive arithmetic task delivered via the Quick Brain application (Brainsoft Apps). Participants in stress conditions completed a continuous sequence of timed mathematical challenges intended to elicit sustained performance pressure and cognitive load. The task battery included Quick Math (rapid arithmetic operations), True/False Math (speeded verification of numerical statements), Math Balance (equivalence-solving under time constraints), Schulte Table (rapid visual–spatial scanning), and Calculate & Input (fast calculation and motor response). All modules operated under strict time limits, and incorrect answers triggered an immediate restart of the problem set, maintaining persistent cognitive demand and limiting performance relief.
To confirm the effectiveness of stress manipulation, a physiological marker was collected after the induction procedure. Salivary cortisol samples were obtained immediately after task completion. Participants in the control condition did not complete the stress-inducing task. Instead, they remained in a virtual waiting room for an equivalent duration, wearing noise-canceling headphones to eliminate auditory distractions and avoid any unintended exposure to stress-evoking stimuli.
2.7. Cortisol Assay
Immediately after the completion of the final trial, salivary samples were collected to assess activation of the HPA axis. Samples were obtained using passive drool into polypropylene tubes of 5 mL (Eppendorf Tubes®, Cat. 0030119401, Eppendorf AG, Hamburg, Germany). All samples were collected within a 2 min window following task termination, between 9:00 and 10:00 a.m., to minimize circadian variability and capture the acute stress-related cortisol response. Following collection, samples were immediately placed on ice, transported to the laboratory, and centrifuged at 3000 rpm for 15 min to remove cellular debris. The clarified supernatant was aliquoted into labeled microtubes and stored at −20 °C until batch analysis.
Cortisol concentrations were determined using a competitive enzyme immunoassay (Cortisol ELISA Kit, ADI-900-071; Enzo Life Sciences, Farmingdale, NY, USA), following the manufacturer’s protocol. Briefly, samples and standards were brought to room temperature, pipetted into antibody-coated wells, and incubated with enzyme conjugate. After washing to remove unbound components, substrate solution was added to initiate color development, and absorbance was read at 450 nm using a microplate spectrophotometer (Agilent BioTek Epoch 2, Agilent Technologies, Santa Clara, CA, USA).
2.8. The VRAM Task
Cognitive performance was assessed using the NeuroHM virtual radial eight-arm maze task. Before the experimental session, all participants received a standardized tutorial designed to habituate them to the immersive environment and to provide instruction on the use of the hand-held controllers for navigating the maze and identifying exit doors, ensuring that task demands were fully understood prior to testing. Each participant completed five consecutive trials, each lasting 60 s, with a two-minute resting interval between trials (control group) or stress induction interval (stress group). The primary objective of the task was to locate the four exit doors within a maximum duration of 60 s per trial, minimizing the number of errors by employing mnemonic and spatial mapping strategies. The main dependent variables in NeuroHM were quantified through three behavioral parameters: (1) latency, defined as the total time required to complete the maze; (2) reference memory errors, defined as the number of first entries into arms that did not contain an exit; and (3) working memory errors, defined as the number of re-entries into previously visited arms that did not contain an exit. All behavioral variables were automatically recorded within the virtual environment for each of the five trials completed by every participant.
2.9. Statistical Analysis
All statistical analyses were conducted using GraphPad Prism (version 8.0; GraphPad Software, San Diego, CA, USA). Descriptive statistics are reported as mean ± standard error of the mean (SEM). Trial-by-trial performance across the five sessions was analyzed using ANOVA, and Sidak’s post hoc multiple comparison test was applied to identify specific differences. In addition, mean values of the dependent variables were compared between the control and stress groups using independent-samples t-tests. A significance level of p < 0.05 was used for all analyses.
3. Results
Before performing the inferential analyses, all statistical assumptions were systematically evaluated to ensure the validity of the results. Normality of residuals was assessed using the Shapiro–Wilk test together with visual inspection of Q–Q plots, which confirmed an approximately normal distribution. Sphericity was examined through the software’s default tests (sphericity check within GraphPad), and in cases where the assumption was not met, the Geisser–Greenhouse correction was applied.
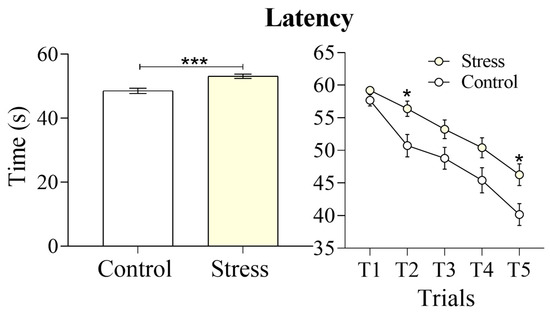
The ANOVA revealed a significant main effect of cognitive stress, F(4,312) = 44.40, p = 0.001, η2 = 0.10, IC95% [1.750, 7.360]. Sidak post hoc comparisons indicated that participants in the stress condition exhibited significantly longer latencies during the second trial 56.39 ± 1.174 vs. 50.73 ± 1.709, p = 0.03, and the fifth trial 46.27 ± 1.668 vs. 40.16 ± 1.680, p = 0.02. When all trials were analyzed together, a Student’s t-test showed that the stress-induced condition scored higher overall than the control group 53.11 ± 0.66 vs. 48.55 ± 0.82; t (98) = 4.290, p = 0.001, d = 0.86 IC95% [2.467, 6.642] (Figure 3). Despite this impairment, both groups demonstrated a progressive reduction in completion time across successive trials, indicating effective learning of the task rules and successful identification of the four exit doors.
Figure 3.
Latency. Time employed to complete the maze. Values correspond to group means with S.E.M, as error bars for the control and stress conditions. The left panel illustrates the overall time employed to complete the task across all trials. The right panel represents trial-by-trial performance, showing group differences in learning dynamics across the five consecutive trials. (* p < 0.05, *** p < 0.001).
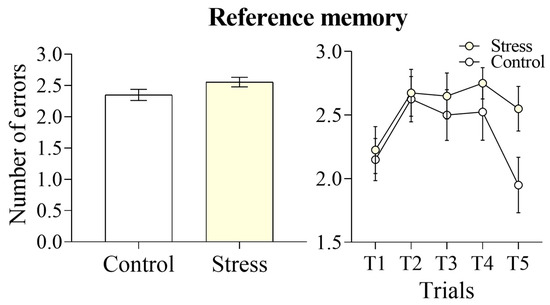
When we evaluated reference memory, the ANOVA did not reveal significant differences between groups, F(4,312) = 3.629, p = 0.8686, η2 = 0.01, IC95% [−0.092, 0.5324] and t-student analysis t (98) = 1.746, p = 0.08, d = 0.35 IC95% [−0.025, 0.435] (Figure 4). This result indicates that both stressed and control participants were equally capable of acquiring long-term knowledge regarding the location of the correct exits.
Figure 4.
Reference memory. The number of initial entries into arms that did not contain an exit. Values correspond to group means with S.E.M, as error bars for the control and stress conditions. The left panel illustrates the total errors during the task. The right panel shows trial-by-trial performance, showing group differences in reference memory across the five consecutive trials.
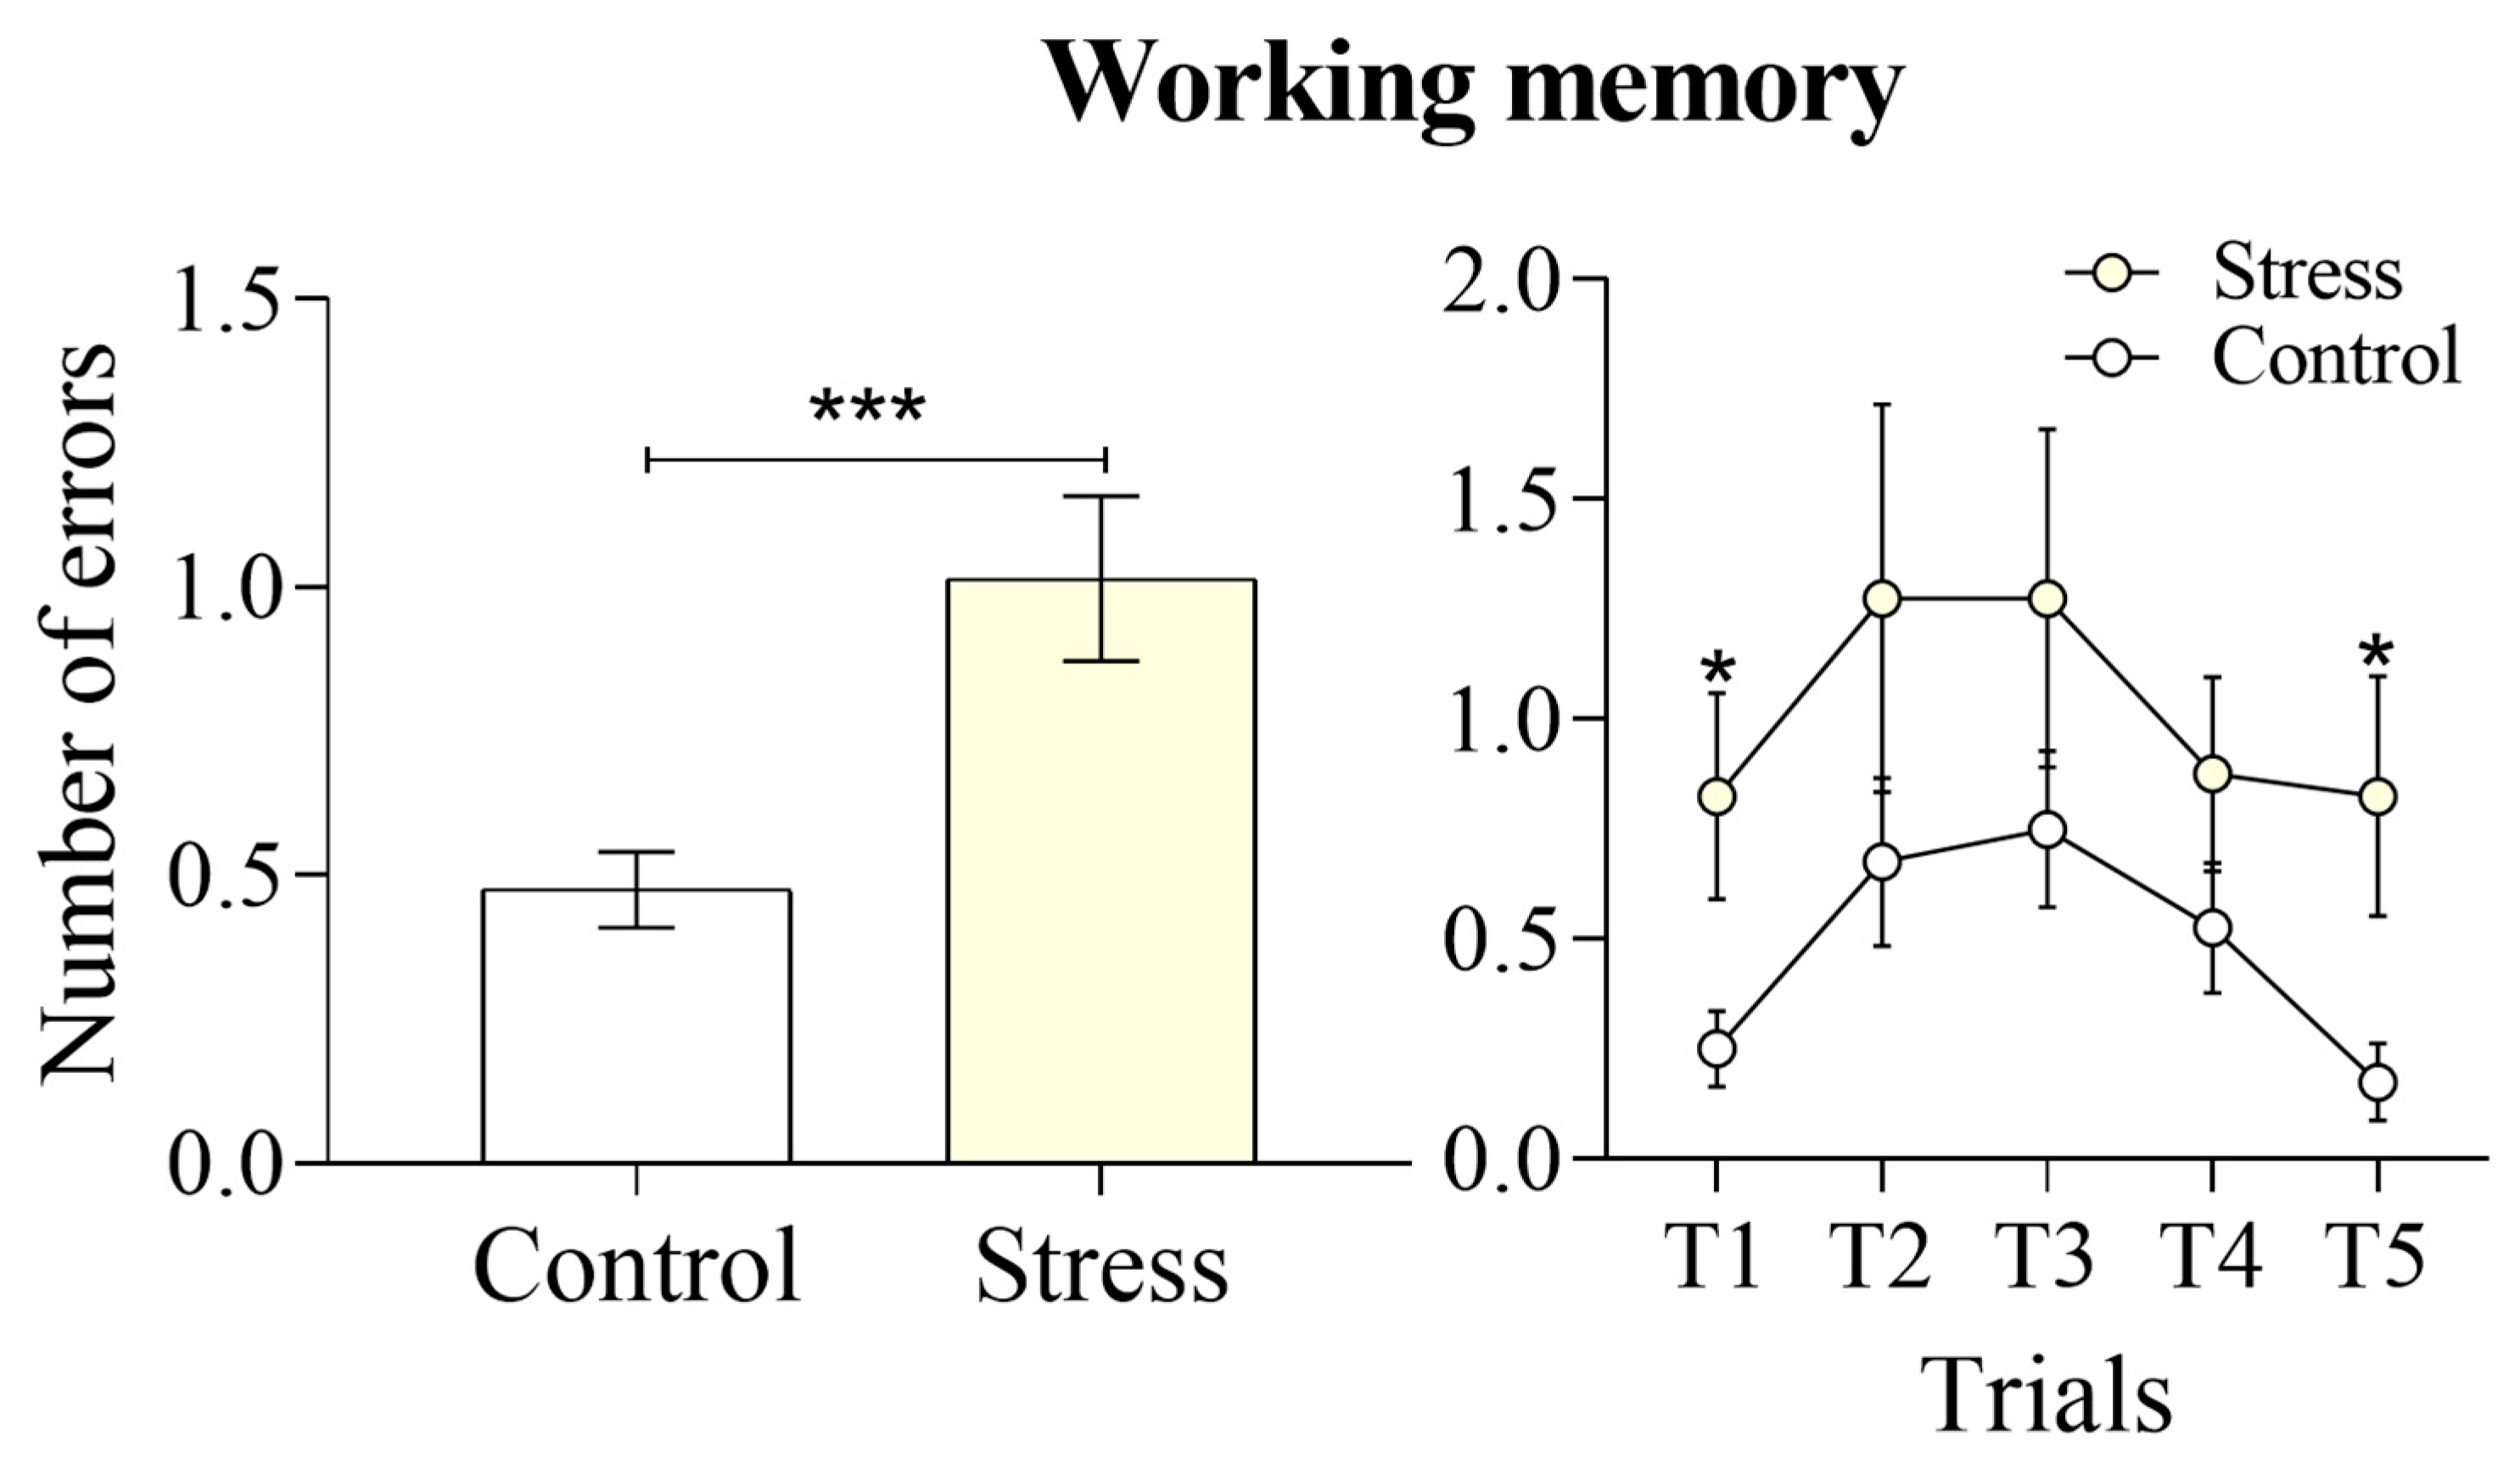
In contrast, analysis of working memory revealed a significant impairment in the stress group, F(4,312) = 2.445, p = 0.001, η2 = 0.045, IC95% [0.106, 0.973]. Sidak post hoc tests showed that stressed participants committed more working memory errors, particularly in the first trial 0.825 ± 0.2345 vs. 0.250 ± 0.085; p = 0.03, and the fifth trial 0.825 ± 0.2724 vs. 0.1750 ± 0.086; p = 0.03. When all trials were considered together, a Student’s t-test confirmed higher overall error rates in the stress group compared with controls 1.015 ± 0.14 vs. 0.47 ± 0.66; t (98) = 3.416, p = 0.001, d = 0.68, IC95% [0.229, 0.850] as shown in Figure 5.
Figure 5.
Working memory. The number of re-entries into arms that did not contain an exit. Values correspond to group means with S.E.M, as error bars for the control and stress conditions. The left panel illustrates the total errors during the task. The right panel shows trial-by-trial performance, showing group differences in reference memory across the five consecutive trials. (* p < 0.05, *** p < 0.001).
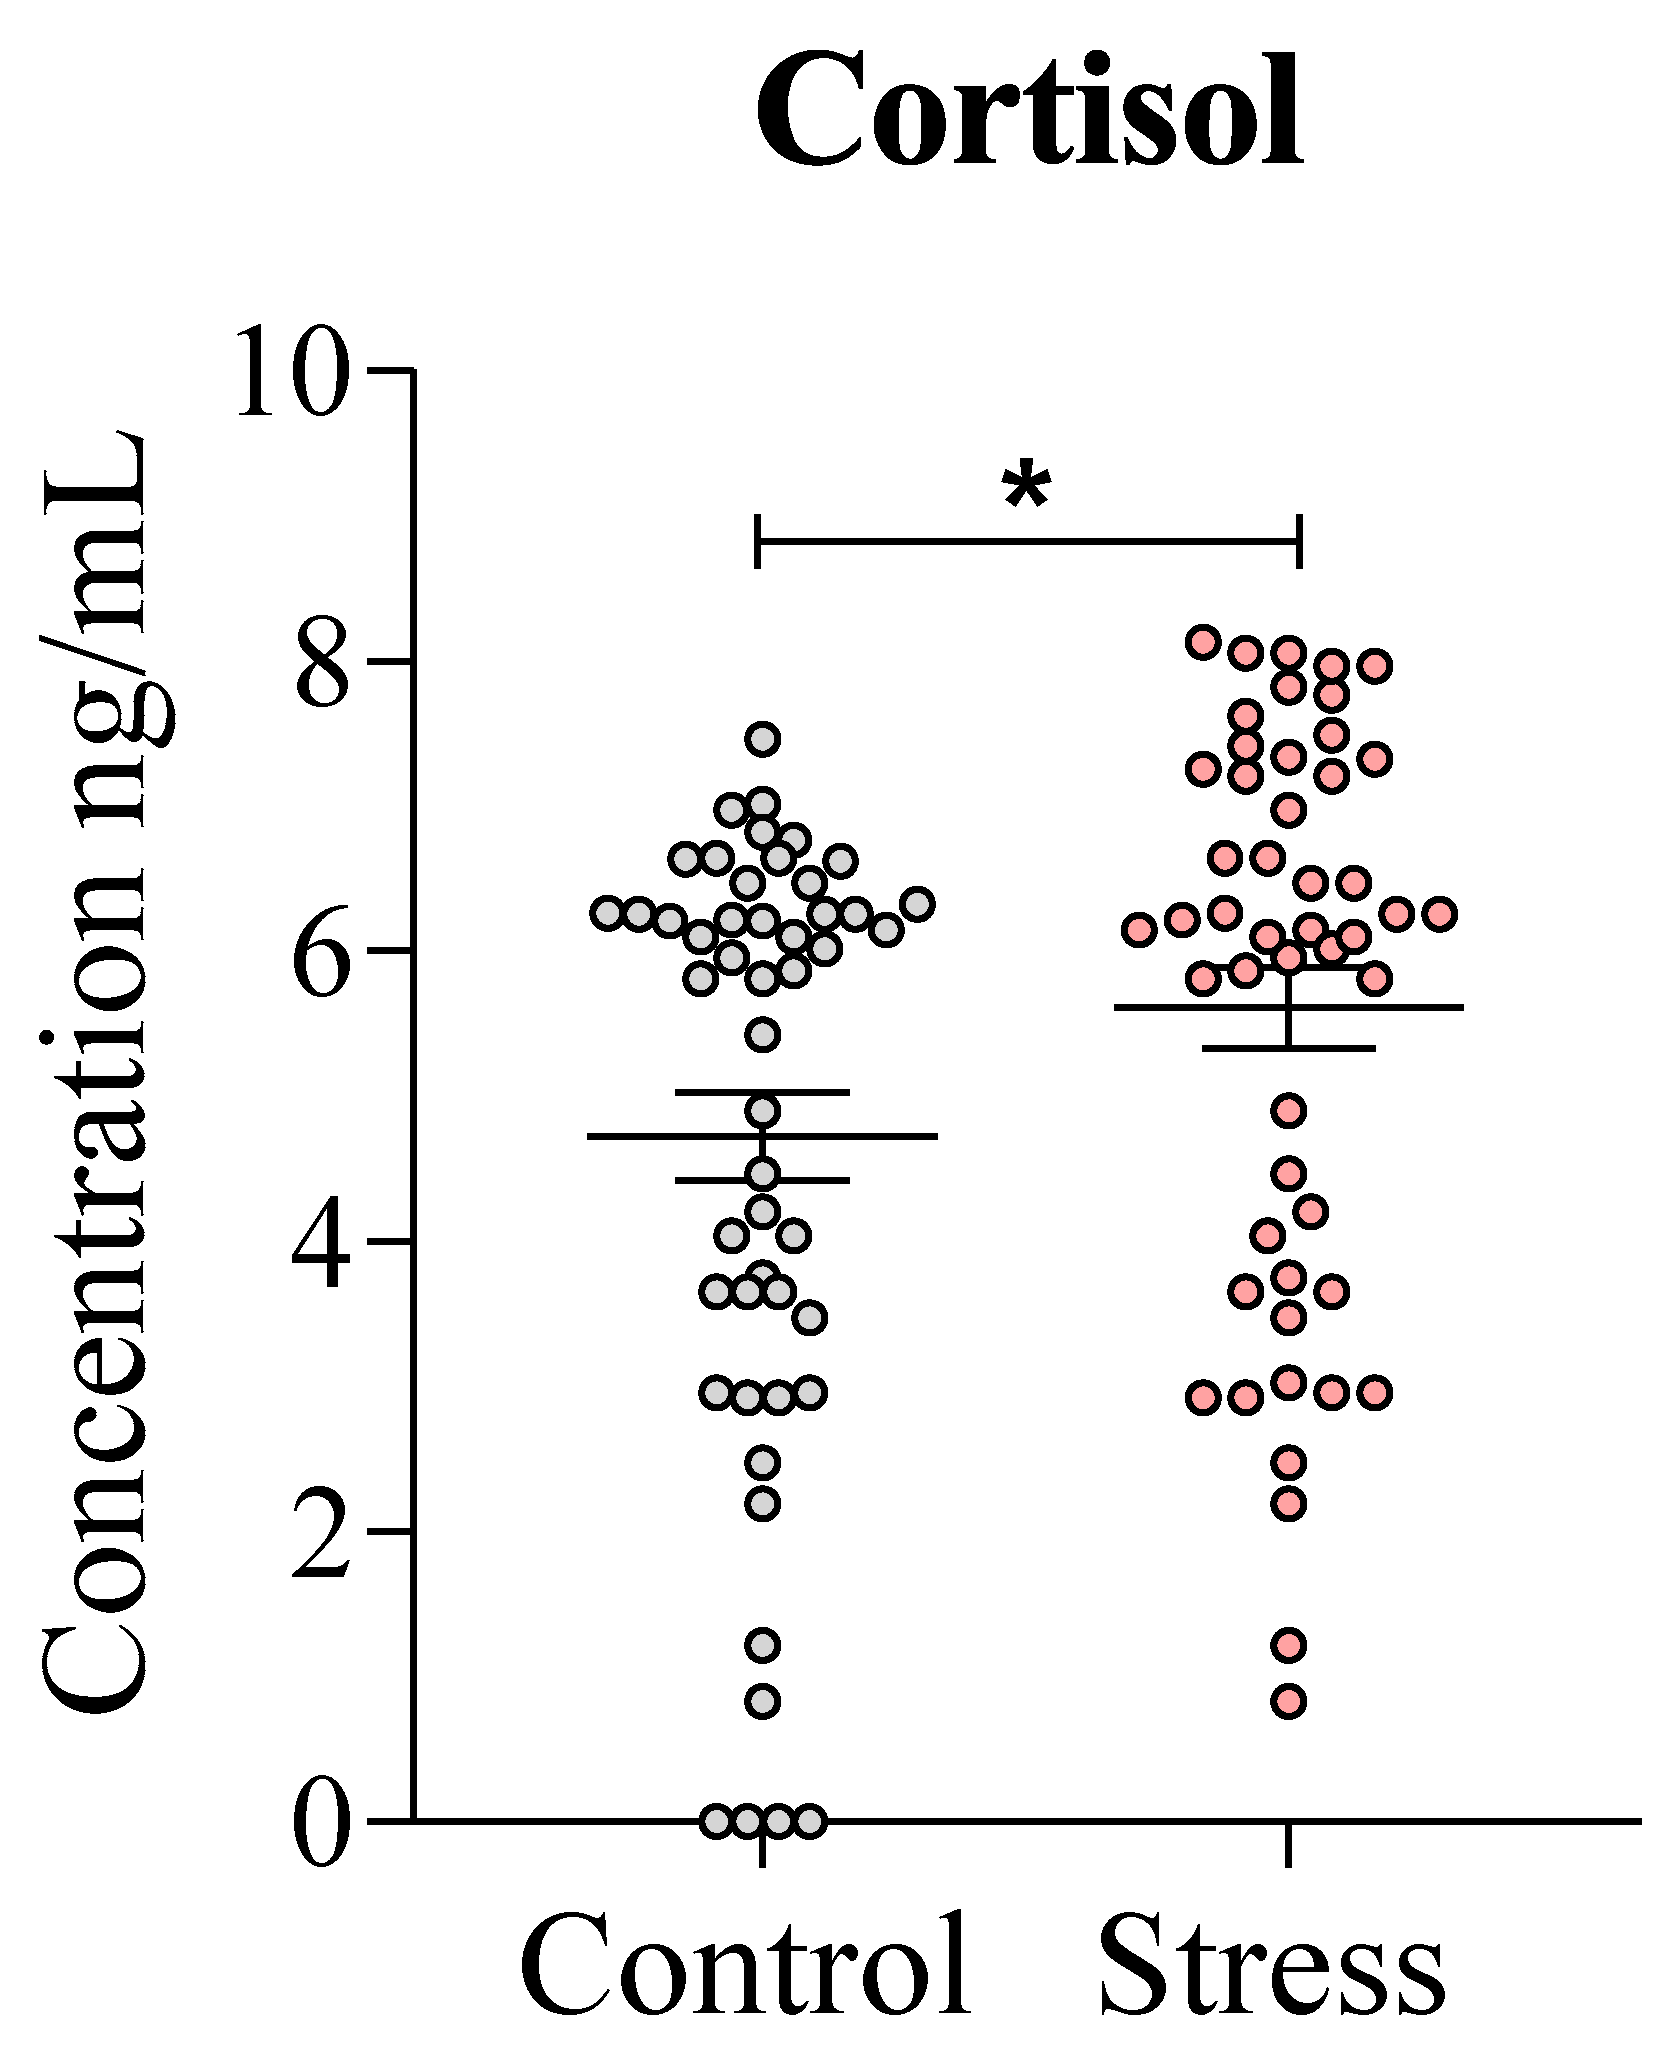
Finally, analysis of salivary cortisol concentrations confirmed the effectiveness of the stress induction procedure. An independent t-test showed that the stress group exhibited significantly higher cortisol levels compared with the control group 5.60 ± 0.28 vs. 4.72 ± 0.30; t (98) = 2.142, p = 0.03, d = 0.43, IC95% [0.065, 1.708], as shown in Figure 6.
Figure 6.
Salivary cortisol concentrations. Values correspond to group means with S.E.M, as error bars for the control and stress conditions. (* p < 0.05).
4. Discussion
The results confirmed that the laboratory stress protocol successfully elicited a physiological stress response, as reflected by a significant increase in salivary cortisol concentrations among participants in the stress condition. As hypothesized, acute stress exposure led to a deterioration in cognitive performance, characterized by longer maze completion times and a higher number of working memory errors.
The observed data support the hypothesis that acute stress induces a shift in navigation strategies from flexible, cognitive, hippocampal-dependent mechanisms toward more rigid, habit-based, cortico-striatal strategies [38,39]. This finding aligns with previous studies reporting that stress alters the balance between memory systems, favoring procedural responses over spatial or declarative strategies [6,40,41,42]. Here, stressors were applied during the navigation task itself, including the intertrial intervals, suggesting that both the HPA and SAM axis were simultaneously active [43]. Consistent with this interpretation, participants in the stress group exhibited significantly higher salivary cortisol [44] concentrations following task completion.
The interaction between cognitive and affective cortical networks and the HPA axis suggests that stress-related hormonal activity can directly modulate cognition. One plausible mechanism for this shift involves catecholaminergic signaling within the basolateral amygdala (BLA), which promotes a transition from hippocampal-based memory retrieval toward striatal-based memory encoding [45]. Catecholamines such as noradrenaline rapidly enhance excitatory transmission and synaptic plasticity through β-adrenergic receptors, while α-adrenergic receptors also contribute to stress-induced modulation. In parallel, corticotropin-releasing factor (CRF) acting through CRF1 receptors increases limbic excitability and promotes glutamate release, thereby enabling rapid structural and synaptic changing in hippocampal CA1 neurons [46,47]. Furthermore, catecholamines and neuropeptides exert rapid effects within minutes through membrane-bound receptors, whereas corticosteroids act more slowly by binding to intracellular glucocorticoid receptors that regulate gene transcription [48]. Consequently, stress mediators can alter neuronal activity and plasticity over a broad temporal range—from minutes to hours to explain why brief stress exposure can influence memory management. In the current study, we observed a transient increase in working memory errors in the stress group, likely reflecting prefrontal cortical involvement and the short-term impact of acute stress on executive processes [45].
Our research tool is meaningful because it introduces an immersive virtual reality version of the radial arm maze specifically designed for human participants, addressing the ecological and methodological limitations of previous two-dimensional or non-immersive adaptations. Earlier studies employing virtual mazes for humans often relied on flat monitors or simplified environments [49,50,51], which restricted the participant’s sense of presence and reduced engagement of spatial navigation systems. More recently, Kim, Park, and Kim (2018) implemented a head-mounted display version of the radial arm maze to assess spatial learning and memory in humans, demonstrating that virtual navigation tasks can successfully reproduce spatial learning patterns similar to those observed in rodents [52]. However, their design remained limited in environmental complexity and interactivity, highlighting the need for more immersive and ecologically valid approaches.
Recent advances in virtual navigation tasks for animal models further support the validity of immersive spatial paradigms. For example, Islam et al. [53] demonstrated that adult zebrafish can successfully acquire Morris Water Maze-like learning within a two-dimensional virtual reality system, highlighting the feasibility of modeling complex spatial behaviors in non-mammalian species. Similarly, Chen et al. [54] showed that head-restrained mice navigating a virtual open arena exhibit robust spatial cell firing patterns comparable to real-world exploration, providing strong evidence that VR environments can reliably engage hippocampal-dependent spatial circuits. These studies demonstrate the translational value of VR-based navigation assays across species and further support the use of human VR paradigms such as NeuroHM to interrogate stress-related disruptions in hippocampal-dependent memory.
The NeuroHM task builds upon and extends these developments by providing a fully interactive three-dimensional environment that allows natural exploration through a head-mounted display, enhancing both ecological validity and the realism of spatial cues. We developed a fully immersive virtual reality maze that offers a 360-degree navigational experience, allowing participants to move freely and explore the environment. The maze design faithfully replicates the classical configuration of the radial arm maze, incorporating elevated walls along each corridor to recreate the perception of enclosed escape arms and maintain spatial orientation. The central platform was intentionally enlarged and designed as an active navigational area rather than a simple transition zone, allowing participants to integrate distal cues into their route-planning strategies. Furthermore, the maze was specifically configured to support real-time data acquisition, thereby allowing for immediate retrieval and comprehensive analysis of behavioral metrics by researchers. The NeuroHM paradigm also holds potential for adaptation to clinical populations with stress-related cognitive dysfunction. Virtual reality tasks have been successfully implemented in patients with PTSD, anxiety disorders, and mild cognitive impairment to assess hippocampal-dependent memory, attentional control, and stress responsivity [55,56,57]. Furthermore, coupling the paradigm with portable neuroimaging tools, including EEG or fNIRS, could help identify neural signatures of altered hippocampal–prefrontal interaction commonly observed in stress-related disorders.
Potential confounding factors must also be considered when interpreting the present findings. Gender differences may influence both stress responsivity and navigation behavior, as males and females often show distinct patterns of HPA axis activation and differential engagement of hippocampal versus striatal systems [58]. These differences could alter the magnitude of cortisol reactivity as well as the type of spatial strategies employed under stress. Similarly, prior gaming or VR experience may confer an advantage by enhancing visuospatial processing, improving sensorimotor coordination, and reducing novelty-related arousal, thereby facilitating maze performance independent of stress manipulation [59]. Baseline anxiety levels represent another relevant source of variability: elevated anxiety can amplify physiological arousal, bias attentional resources, and impair prefrontal executive function, potentially increasing working memory errors and modifying navigation strategies. As these factors were not systematically assessed, they may have contributed to inter-individual variability in both behavioral and physiological outcomes.
The principal limitation of the present study is its modest sample size, which reduces statistical power and restricts the generalizability of the results. Although pilot-stage VR cognitive studies commonly rely on similar sample sizes, larger and more demographically diverse cohorts are necessary to confirm the robustness and external validity of the present findings. Large-scale digital navigation research, such as the Sea Hero Quest dataset analyzed by Coutrot et al. [60], which included more than two million participants worldwide, demonstrates the importance of broad population sampling for characterizing spatial learning variability across individuals. A second limitation concerns the restricted set of physiological stress markers. Although salivary cortisol was assessed, additional measures, such as heart rate variability, electrodermal activity, or validated subjective anxiety scales, would provide a more comprehensive evaluation of acute stress responses [61]. Future studies should incorporate multi-modal physiological assessments to more precisely characterize stress reactivity and its cognitive consequences. Another limitation is the absence of complementary neuropsychological assessments. Including standardized cognitive batteries would enable direct comparisons between traditional measures of memory and performance on immersive spatial navigation tasks, providing stronger construct validity. It is also important to consider that the technological characteristics of different virtual reality systems (display resolution, field of view, frame rate, and motion tracking precision), may influence the encoding and retrieval of spatial information. These variations could account for discrepancies among studies employing different hardware or software configurations. Furthermore, future investigations could integrate neuroimaging and electrophysiological techniques to examine the neural correlations of virtual navigation under experimental conditions. Moreover, future research should experimentally assess individuals with clinically diagnosed cognitive impairments. These evaluations would yield critical evidence on the sensitivity of the NeuroHM task in detecting hippocampal-dependent dysfunctions and would further substantiate its utility as a diagnostic and monitoring instrument. Accordingly, future work will address these limitations by expanding sample size and demographic breadth, incorporating autonomic stress markers such as HRV and EDA alongside validated anxiety scales, and adding a complementary standardized neuropsychological battery to directly benchmark VR-based spatial memory performance against traditional cognitive measures.
5. Conclusions
The present pilot study introduces NeuroHM as a novel virtual reality adaptation of the radial eight-arm maze for assessing human spatial learning and memory. Although preliminary, the results indicate that the system is sensitive to stress-related performance changes. Given the limited sample size, the exploratory nature of the design, and the use of a single physiological stress marker, the conclusions should be interpreted cautiously. Nevertheless, these initial findings suggest that NeuroHM has potential as a complementary tool for cognitive assessment and as a platform for future translational research in stress and mental health. Replication with larger, more diverse samples and expanded physiological and neuropsychological measures will be essential to establish its robustness and clinical utility.
Author Contributions
Conceptualization, D.F.-Q.; methodology, P.A.A.-D., D.E.M.-F. and D.F.-Q.; software, P.A.A.-D.; validation, D.E.M.-F. and D.F.-Q.; formal analysis, P.A.A.-D. and D.E.M.-F.; investigation, P.A.A.-D., D.E.M.-F. and D.F.-Q.; resources, P.A.A.-D.; data curation, D.E.M.-F.; writing—original draft preparation, P.A.A.-D. and D.E.M.-F.; writing—review and editing, D.F.-Q.; visualization, D.F.-Q.; supervision, D.F.-Q.; project administration, D.F.-Q.; funding acquisition, D.F.-Q. All authors have read and agreed to the published version of the manuscript.
Funding
This research was funded by the University of Guadalajara, through the “Programa de Apoyo a la Mejora en las Condiciones de Producción de las Personas Integrantes del SNII y SNCA (PROSNII) 2025” grant number (U006EST).
Institutional Review Board Statement
The study was conducted in accordance with the Declaration of Helsinki and approved by the Ethics Committee of the University of Guadalajara (protocol code CI-01225 and date of approval 1 January 2025).
Informed Consent Statement
Informed consent was obtained from all subjects involved in the study.
Data Availability Statement
The original contributions presented in this study are included in the article. Further inquiries can be directed to the corresponding authors.
Acknowledgments
We thanks to Neuroscience Department of the University of Guadalajara.
Conflicts of Interest
The authors declare no conflicts of interest.
Abbreviations
The following abbreviations are used in this manuscript:
| CRF | Corticotropin-Releasing Factor |
| EEG | Electroencephalogram |
| fNIRS | Functional Near-Infrared Spectroscopy |
| HPA | Hypothalamic Pituitary Adrenal axis |
| MWM | Morris Water Maze |
| RAM | Radial Arm Maze |
| SAM | Sympathetic–Adrenal–Medullary axis |
| VR | Virtual Reality |
References
- Goldstein, D.S.; Kopin, I.J. Evolution of Concepts of Stress. Stress 2007, 10, 109–120. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- van Herk, L.; Schilder, F.P.M.; de Weijer, A.D.; Bruinsma, B.; Geuze, E. Heightened SAM- and HPA-Axis Activity during Acute Stress Impairs Decision-Making: A Systematic Review on Underlying Neuropharmacological Mechanisms. Neurobiol. Stress 2024, 31, 100659. [Google Scholar] [CrossRef] [Scilit]
- Guo, X.; Wang, Y.; Kan, Y.; Wu, M.; Ball, L.J.; Duan, H. The HPA and SAM Axis Mediate the Impairment of Creativity under Stress. Psychophysiology 2024, 61, e14472. [Google Scholar] [CrossRef] [Scilit]
- Sherman, B.E.; Harris, B.B.; Turk-Browne, N.B.; Sinha, R.; Goldfarb, E.V. Hippocampal Mechanisms Support Cortisol-Induced Memory Enhancements. J. Neurosci. 2023, 43, 7198–7212. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kremen, W.S.; Panizzon, M.S.; Lyons, M.J.; Franz, C.E. Cortisol and Brain: Beyond the Hippocampus. Biol. Psychiatry 2011, 69, e9; author reply e11. [Google Scholar] [CrossRef] [Scilit]
- Fernández-Quezada, D.; Moran-Torres, D.; Luquin, S.; Ruvalcaba-Delgadillo, Y.; García-Estrada, J.; Jáuregui-Huerta, F. Male/Female Differences in Radial Arm Water Maze Execution After Chronic Exposure to Noise. Noise Health 2019, 21, 25–34. [Google Scholar] [CrossRef] [Scilit]
- Sazma, M.A.; Shields, G.S.; Yonelinas, A.P. The Effects of Post-Encoding Stress and Glucocorticoids on Episodic Memory in Humans and Rodents. Brain Cogn. 2019, 133, 12–23. [Google Scholar] [CrossRef] [Scilit]
- Bhakta, A.; Gavini, K.; Yang, E.; Lyman-Henley, L.; Parameshwaran, K. Chronic Traumatic Stress Impairs Memory in Mice: Potential Roles of Acetylcholine, Neuroinflammation and Corticotropin Releasing Factor Expression in the Hippocampus. Behav. Brain Res. 2017, 335, 32–40. [Google Scholar] [CrossRef] [Scilit]
- Lupien, S.J.; Fiocco, A.; Wan, N.; Maheu, F.; Lord, C.; Schramek, T.; Tu, M.T. Stress Hormones and Human Memory Function across the Lifespan. Psychoneuroendocrinology 2005, 30, 225–242. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Quaedflieg, C.W.E.M.; Schneider, T.R.; Daume, J.; Engel, A.K.; Schwabe, L. Stress Impairs Intentional Memory Control through Altered Theta Oscillations in Lateral Parietal Cortex. J. Neurosci. 2020, 40, 7739–7748. [Google Scholar] [CrossRef] [Scilit]
- Nitschke, J.P.; Giorgio, L.-M.; Zaborowska, O.; Sheldon, S. Acute Psychosocial Stress during Retrieval Impairs Pattern Separation Processes on an Episodic Memory Task. Stress 2020, 23, 437–443. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Heinbockel, H.; Wagner, A.D.; Schwabe, L. Post-Retrieval Stress Impairs Subsequent Memory Depending on Hippocampal Memory Trace Reinstatement during Reactivation. Sci. Adv. 2024, 10, eadm7504. [Google Scholar] [CrossRef] [Scilit]
- Schwabe, L.; Hermans, E.J.; Joëls, M.; Roozendaal, B. Mechanisms of Memory under Stress. Neuron 2022, 110, 1450–1467. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Schwabe, L.; Wolf, O.T. Stress Prompts Habit Behavior in Humans. J. Neurosci. 2009, 29, 7191–7198. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- van Gerven, D.J.H.; Ferguson, T.; Skelton, R.W. Acute Stress Switches Spatial Navigation Strategy from Egocentric to Allocentric in a Virtual Morris Water Maze. Neurobiol. Learn. Mem. 2016, 132, 29–39. [Google Scholar] [CrossRef] [Scilit]
- Burgess, N.; Maguire, E.A.; O’Keefe, J. The Human Hippocampus and Spatial and Episodic Memory. Neuron 2002, 35, 625–641. [Google Scholar] [CrossRef] [Scilit]
- Santos-Carrasco, D.; Casa, L.G.D.L. Spanish Validation of the Maastricht Acute Stress Test (MAST): A Cost-Effective Stress Induction Protocol. Span. J. Psychol. 2025, 28, e1. [Google Scholar] [CrossRef] [Scilit]
- Ghosh, R.; Deb, N.; Sengupta, K.; Phukan, A.; Choudhury, N.; Kashyap, S.; Phadikar, S.; Saha, R.; Das, P.; Sinha, N.; et al. SAM 40: Dataset of 40 Subject EEG Recordings to Monitor the Induced-Stress While Performing Stroop Color-Word Test, Arithmetic Task, and Mirror Image Recognition Task. Data Brief 2022, 40, 107772. [Google Scholar] [CrossRef] [Scilit]
- Kirschbaum, C.; Pirke, K.M.; Hellhammer, D.H. The ’Trier Social Stress Test’—A Tool for Investigating Psychobiological Stress Responses in a Laboratory Setting. Neuropsychobiology 1993, 28, 76–81. [Google Scholar] [CrossRef] [Scilit]
- Foley, P.; Kirschbaum, C. Human Hypothalamus-Pituitary-Adrenal Axis Responses to Acute Psychosocial Stress in Laboratory Settings. Neurosci. Biobehav. Rev. 2010, 35, 91–96. [Google Scholar] [CrossRef] [Scilit]
- Brandeis, R.; Brandys, Y.; Yehuda, S. The Use of the Morris Water Maze in the Study of Memory and Learning. Int. J. Neurosci. 1989, 48, 29–69. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dale, R.H. Spatial and Temporal Response Patterns on the Eight-Arm Radial Maze. Physiol. Behav. 1986, 36, 787–790. [Google Scholar] [CrossRef] [Scilit]
- Smith, S.A. Virtual Reality in Episodic Memory Research: A Review. Psychon. Bull. Rev. 2019, 26, 1213–1237. [Google Scholar] [CrossRef] [Scilit]
- Cimadevilla, J.M.; Nori, R.; Piccardi, L. Application of Virtual Reality in Spatial Memory. Brain Sci. 2023, 13, 1621. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Brookes, J.; Warburton, M.; Alghadier, M.; Mon-Williams, M.; Mushtaq, F. Studying Human Behavior with Virtual Reality: The Unity Experiment Framework. Behav. Res. Methods 2020, 52, 455–463. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sagaspe, P.; Amieva, H.; Dartigues, J.-F.; Olive, J.; de la Rivière, J.-B.; Chartier, C.; Taillard, J.; Philip, P. Validity and Diagnostic Performance of a Virtual Reality-Based Supermarket Application “MEMOSHOP” for Assessing Episodic Memory in Normal and Pathological Aging. Digit. Health 2023, 9, 20552076231218808. [Google Scholar] [CrossRef] [Scilit]
- Spieker, E.A.; Astur, R.S.; West, J.T.; Griego, J.A.; Rowland, L.M. Spatial Memory Deficits in a Virtual Reality Eight-Arm Radial Maze in Schizophrenia. Schizophr. Res. 2012, 135, 84–89. [Google Scholar] [CrossRef] [Scilit]
- Palombi, T.; Mandolesi, L.; Alivernini, F.; Chirico, A.; Lucidi, F. Application of Real and Virtual Radial Arm Maze Task in Human. Brain Sci. 2022, 12, 468. [Google Scholar] [CrossRef] [Scilit]
- Sánchez-Escudero, J.P.; Galvis-Herrera, A.M.; Sánchez-Trujillo, D.; Torres-López, L.C.; Kennedy, C.J.; Aguirre-Acevedo, D.C.; Garcia-Barrera, M.A.; Trujillo, N. Virtual Reality and Serious Videogame-Based Instruments for Assessing Spatial Navigation in Alzheimer’s Disease: A Systematic Review of Psychometric Properties. Neuropsychol. Rev. 2025, 35, 77–101. [Google Scholar] [CrossRef] [Scilit]
- Laczó, J.; Andel, R.; Vyhnalek, M.; Vlcek, K.; Magerova, H.; Varjassyova, A.; Tolar, M.; Hort, J. Human Analogue of the Morris Water Maze for Testing Subjects at Risk of Alzheimer’s Disease. Neurodegener. Dis. 2010, 7, 148–152. [Google Scholar] [CrossRef] [Scilit]
- Park, J.-H. Can the Virtual Reality-Based Spatial Memory Test Better Discriminate Mild Cognitive Impairment than Neuropsychological Assessment? Int. J. Environ. Res. Public Health 2022, 19, 9950. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wallet, G.; Sauzéon, H.; Pala, P.A.; Larrue, F.; Zheng, X.; N’Kaoua, B. Virtual/Real Transfer of Spatial Knowledge: Benefit from Visual Fidelity Provided in a Virtual Environment and Impact of Active Navigation. Cyberpsychol. Behav. Soc. Netw. 2011, 14, 417–423. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ruddle, R.A.; Volkova, E.; Mohler, B.; Bülthoff, H.H. The Effect of Landmark and Body-Based Sensory Information on Route Knowledge. Mem. Cogn. 2011, 39, 686–699. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dehn, L.B.; Kater, L.; Piefke, M.; Botsch, M.; Driessen, M.; Beblo, T. Training in a Comprehensive Everyday-like Virtual Reality Environment Compared to Computerized Cognitive Training for Patients with Depression. Comput. Hum. Behav. 2018, 79, 40–52. [Google Scholar] [CrossRef] [Scilit]
- Shen, J.; Koterba, C.; Samora, J.; Leonard, J.; Li, R.; Shi, J.; Yeates, K.O.; Xiang, H.; Taylor, G. Usability and Validity of a VR Cognitive Assessment Tool for Pediatric TBI. Rehabil. Psychol. 2022, 67, 587–596. [Google Scholar] [CrossRef] [Scilit]
- Jespersen, A.E.; Lumbye, A.; Vinberg, M.; Glenthøj, L.; Nordentoft, M.; Wæhrens, E.E.; Knudsen, G.M.; Makransky, G.; Miskowiak, K.W. Effect of Immersive Virtual Reality-Based Cognitive Remediation in Patients with Mood or Psychosis Spectrum Disorders: Study Protocol for a Randomized, Controlled, Double-Blinded Trial. Trials 2024, 25, 82. [Google Scholar] [CrossRef] [Scilit]
- Garrett, B.; Tao, G.; Taverner, T.; Gromala, D.; Musoke, R.; Sun, C.; Shaw, C.D.; Cordingley, E. An Exploratory Randomized Controlled Trial of Virtual Reality as a Non-Pharmacological Adjunctive Intervention for Adults with Chronic Cancer-Related Pain. BMC Digit. Health 2024, 2, 28. [Google Scholar] [CrossRef] [Scilit]
- Brunyé, T.T.; Wood, M.D.; Houck, L.A.; Taylor, H.A. The Path More Travelled: Time Pressure Increases Reliance on Familiar Route-Based Strategies during Navigation. Q. J. Exp. Psychol. 2017, 70, 1439–1452. [Google Scholar] [CrossRef] [Scilit]
- Brown, T.I.; Gagnon, S.A.; Wagner, A.D. Stress Disrupts Human Hippocampal-Prefrontal Function during Prospective Spatial Navigation and Hinders Flexible Behavior. Curr. Biol. 2020, 30, 1821–1833.e8. [Google Scholar] [CrossRef] [Scilit]
- Boone, A.P.; Bullock, T.; MacLean, M.H.; Santander, T.; Raymer, J.; Stuber, A.; Jimmons, L.; Okafor, G.N.; Grafton, S.T.; Miller, M.B.; et al. Resilience of Navigation Strategy and Efficiency to the Impact of Acute Stress. Spat. Cogn. Comput. 2024, 24, 195–226. [Google Scholar] [CrossRef] [Scilit]
- Meng, F.; Zhang, W. Way-Finding during a Fire Emergency: An Experimental Study in a Virtual Environment. Ergonomics 2014, 57, 816–827. [Google Scholar] [CrossRef] [Scilit]
- Varshney, A.; Munns, M.E.; Kasowski, J.; Zhou, M.; He, C.; Grafton, S.T.; Giesbrecht, B.; Hegarty, M.; Beyeler, M. Stress Affects Navigation Strategies in Immersive Virtual Reality. Sci. Rep. 2024, 14, 5949. [Google Scholar] [CrossRef] [Scilit]
- Richardson, A.E.; VanderKaay Tomasulo, M.M. Influence of Acute Stress on Spatial Tasks in Humans. Physiol. Behav. 2011, 103, 459–466. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hellhammer, D.H.; Wüst, S.; Kudielka, B.M. Salivary Cortisol as a Biomarker in Stress Research. Psychoneuroendocrinology 2009, 34, 163–171. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Barsegyan, A.; Mackenzie, S.M.; Kurose, B.D.; McGaugh, J.L.; Roozendaal, B. Glucocorticoids in the Prefrontal Cortex Enhance Memory Consolidation and Impair Working Memory by a Common Neural Mechanism. Proc. Natl. Acad. Sci. USA 2010, 107, 16655–16660. [Google Scholar] [CrossRef] [Scilit]
- Vandael, D.; Wierda, K.; Vints, K.; Baatsen, P.; De Groef, L.; Moons, L.; Rybakin, V.; Gounko, N.V. Corticotropin-Releasing Factor Induces Functional and Structural Synaptic Remodelling in Acute Stress. Transl. Psychiatry 2021, 11, 378. [Google Scholar] [CrossRef] [Scilit]
- Barsegyan, A.; Mirone, G.; Ronzoni, G.; Guo, C.; Song, Q.; van Kuppeveld, D.; Schut, E.H.S.; Atsak, P.; Teurlings, S.; McGaugh, J.L.; et al. Glucocorticoid Enhancement of Recognition Memory via Basolateral Amygdala-Driven Facilitation of Prelimbic Cortex Interactions. Proc. Natl. Acad. Sci. USA 2019, 116, 7077–7082. [Google Scholar] [CrossRef] [Scilit]
- Joëls, M.; Sarabdjitsingh, R.A.; Karst, H. Unraveling the Time Domains of Corticosteroid Hormone Influences on Brain Activity: Rapid, Slow, and Chronic Modess. Pharmacol. Rev. 2012, 64, 901–938. [Google Scholar] [CrossRef] [Scilit]
- Astur, R.S.; Ortiz, M.L.; Sutherland, R.J. A Characterization of Performance by Men and Women in a Virtual Morris Water Task: A Large and Reliable Sex Difference. Behav. Brain Res. 1998, 93, 185–190. [Google Scholar] [CrossRef] [Scilit]
- Xu, D.; Hao, X.; Wang, Z.; Duan, Y.; Liu, F.; Marsh, R.; Yu, S.; Peterson, B.S. A Virtual Radial Arm Maze for the Study of Multiple Memory Systems in a Functional Magnetic Resonance Imaging Environment. Int. J. Virtual Real. 2012, 11, 63–76. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ben-Zeev, T.; Weiss, I.; Ashri, S.; Heled, Y.; Ketko, I.; Yanovich, R.; Okun, E. Mild Physical Activity Does Not Improve Spatial Learning in a Virtual Environment. Front. Behav. Neurosci. 2020, 14, 584052. [Google Scholar] [CrossRef] [Scilit]
- Kim, H.; Park, J.Y.; Kim, K.K. Spatial Learning and Memory Using a Radial Arm Maze with a Head-Mounted Display. Psychiatry Investig. 2018, 15, 935–944. [Google Scholar] [CrossRef] [Scilit]
- Islam, T.; Torigoe, M.; Tanimoto, Y.; Okamoto, H. Adult Zebrafish Can Learn Morris Water Maze-like Tasks in a Two-Dimensional Virtual Reality System. Cell Rep. Methods 2024, 4, 100863. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, G.; King, J.A.; Lu, Y.; Cacucci, F.; Burgess, N. Spatial Cell Firing during Virtual Navigation of Open Arenas by Head-Restrained Mice. eLife 2018, 7, e34789. [Google Scholar] [CrossRef] [Scilit]
- Tortora, C.; Di Crosta, A.; La Malva, P.; Prete, G.; Ceccato, I.; Mammarella, N.; Di Domenico, A.; Palumbo, R. Virtual Reality and Cognitive Rehabilitation for Older Adults with Mild Cognitive Impairment: A Systematic Review. Ageing Res. Rev. 2024, 93, 102146. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Spytska, L. The Use of Virtual Reality in the Treatment of Mental Disorders Such as Phobias and Post-Traumatic Stress Disorder. SSM Ment. Health 2024, 6, 100351. [Google Scholar] [CrossRef] [Scilit]
- Maples-Keller, J.L.; Bunnell, B.E.; Kim, S.-J.; Rothbaum, B.O. The Use of Virtual Reality Technology in the Treatment of Anxiety and Other Psychiatric Disorders. Harv. Rev. Psychiatry 2017, 25, 103–113. [Google Scholar] [CrossRef] [Scilit]
- Oyola, M.G.; Handa, R.J. Hypothalamic-Pituitary-Adrenal and Hypothalamic-Pituitary-Gonadal Axes: Sex Differences in Regulation of Stress Responsivity. Stress 2017, 20, 476–494. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zioga, T.; Ferentinos, A.; Konsolaki, E.; Nega, C.; Kourtesis, P. Video Game Skills across Diverse Genres and Cognitive Functioning in Early Adulthood: Verbal and Visuospatial Short-Term and Working Memory, Hand–Eye Coordination, and Empathy. Behav. Sci. 2024, 14, 874. [Google Scholar] [CrossRef] [Scilit]
- Coutrot, A.; Silva, R.; Manley, E.; de Cothi, W.; Sami, S.; Bohbot, V.D.; Wiener, J.M.; Hölscher, C.; Dalton, R.C.; Hornberger, M.; et al. Global Determinants of Navigation Ability. Curr. Biol. 2018, 28, 2861–2866.e4. [Google Scholar] [CrossRef] [Scilit]
- Hermans, E.J.; Henckens, M.J.A.G.; Joëls, M.; Fernández, G. Dynamic Adaptation of Large-Scale Brain Networks in Response to Acute Stressors. Trends Neurosci. 2014, 37, 304–314. [Google Scholar] [CrossRef] [Scilit] [PubMed]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.