


Abstract
We investigated the autumn-to-winter evolution of water-mass structure and nutrient concentrations in Funka Bay, southwestern Hokkaido, Japan, from October to February (2012–2019). Hydrographic and biogeochemical profiles show a recurrent seasonal transition from strongly stratified conditions in October, with low surface nutrients and bottom enrichment, to increasingly homogeneous distributions by mid-winter as vertical mixing intensifies. Depth-averaged nutrient concentrations generally decreased from October to December and increased from December to February, except during December 2015–February 2016. To assess whether February nutrient levels can be explained by Oyashio supply alone, we calculated February nutrient concentrations using a two-endmember mixing model (Oyashio endmember and December Funka Bay water) with an additional regeneration term that assumes nutrients consumed during the October–December autumn bloom were fully regenerated during December–February and redistributed by winter mixing. Under this framework, the expected February concentrations agreed with observations in all winters except 2015, when observed nutrients were lower than expected nutrients, consistent with additional biological drawdown after the early onset of the bloom by late February. These results indicate that the pre-bloom winter nutrient environment in Funka Bay is shaped by variable Oyashio intrusion superimposed on seasonal mixing and internal regeneration processes.
1. Introduction
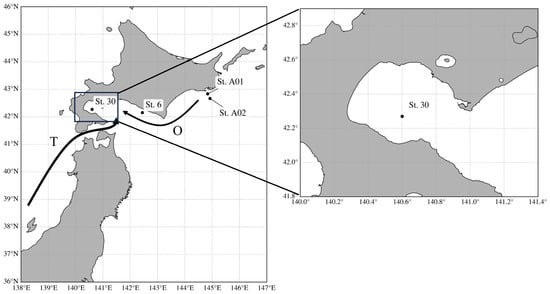
Funka Bay is located in southwestern Hokkaido, Japan (Figure 1). This semi-enclosed inner bay, covering an area of 2485 km2, has a maximum depth of 107 m and features a mouth width of 30.2 km. The bay’s interior is broader than its entrance, and the presence of a sill at the bay mouth facilitates the partial stagnation and modification of water masses within the bay. Because Funka Bay is an important fishing ground and a characteristic subarctic coastal system where seasonal changes in water-mass structure are pronounced, understanding the mechanisms that control its nutrient dynamics and biological productivity is of both industrial and scientific importance [1,2,3,4].
Figure 1.
Tsugaru Current (T; Arrow from Southwast) and Oyashio Current (O; Arrow from Northeast) around Hokkaido, Japan. Station location is shown in the map. We used our original data from St. 30 and St. 6. Data from St. A01 and St. A02 are published on the A Line Monitoring (https://ocean.fra.go.jp/a-line/a-line_index.html; accessed on 22 November 2025).
Funka Bay is seasonally influenced by cold, low-salinity coastal Oyashio water (COW) associated with the Coastal Oyashio system along the Pacific shelf off southern Hokkaido [5,6]. In winter to early spring, this coastal Oyashio water intrudes into Funka Bay (often entering from the northeastern bay near Muroran) and shows marked interannual variability [6]. Seasonal water-mass exchanges occur twice annually: (1) the intrusion of the coastal Oyashio water from winter to spring and (2) the intrusion of the Tsugaru Warm Current (TWC) water from summer to autumn [1,7].
In addition to horizontal exchange, vertical mixing strongly influences the nutrient environment. In winter, the combination of monsoon cold winds and wind-driven turbulence cools and densifies surface waters, deepening the mixed layer and promoting vertical exchange between surface and bottom layers. Through these processes, nutrients regenerated at depth are transported toward the surface and can be utilized by the subsequent spring phytoplankton bloom. In the anomalously warm winter (February) of 2016, when Funka Bay stored a larger amount of ocean heat, a bottom-reaching mixed layer developed because a greater heat content could be removed by surface cooling [8].
Phytoplankton blooms, predominantly composed of diatoms, occur biannually in autumn and spring [9,10,11]. Especially, the areal primary production during spring blooms reaches approximately 1.4 g C m−2 d−1, placing Funka Bay among the most productive coastal systems worldwide [4]. According to the classification system of [12], Funka Bay is categorized as mesotrophic on the basis of its annual primary production.
Following the spring bloom, ammonium concentrations near the bottom layer (80–90 m) have been observed to increase from 2 µmol L−1 in March to 6 µmol L−1 by June [13]. Concurrently, nitrification processes in the bottom layer elevate nitrate and nitrite concentrations from 12 to 20 µmol L−1. The total nitrogen regenerated throughout the water column over this four-month period is estimated at 287.4 mmol N m−2. Assuming the Redfield C:N ratio and that regenerated nitrogen is fully utilized for primary production, this corresponds to approximately 22.8 g C m−2 of production—roughly 34% of the bay’s annual total [13]. These results indicate that regenerated nutrients make a major contribution to the annual production in Funka Bay and underscore the importance of understanding seasonal and interannual variability in nutrient inventories.
The spring bloom alone accounts for approximately 35–50% of the bay’s annual primary production [4,9]. Previous investigations have reported silicate-to-nitrate and nitrate-to-phosphate consumption ratios of 0.9 and 18 during the bloom period, respectively—values broadly consistent with the canonical Redfield ratio [2]. These studies also indicate that nitrate is typically depleted early in the bloom, whereas phosphate and silicic acid often remain at detectable levels [2]. Together, these results suggest that the magnitude and duration of the spring bloom depend sensitively on the pre-bloom nutrient inventories established during the preceding winter.
Most previous work has focused on nutrient dynamics from February onward—just prior to the onset of the spring bloom—and has not explicitly addressed the origin and evolution of nutrients accumulating in the bay from the preceding October. In particular, the relative roles of Oyashio inflow, autumn and winter regeneration, and mid-winter biological uptake in setting the pre-bloom nutrient levels remain unclear. The present study therefore aims to clarify the vertical distribution and temporal evolution of nutrients from October to February, and to identify the sources and processes that control the nutrient inventories supporting the subsequent spring bloom in Funka Bay. To this end, we analyze hydrographic and biogeochemical data collected by the training vessel Ushio Maru of the Faculty of Fisheries, Hokkaido University, for the periods October–December and October–February between 2012–2016 and 2018–2019. We focus on linking the October–February changes in water-mass structure and nutrient concentrations to the known characteristics of the spring bloom, thereby evaluating the extent to which winter processes precondition spring primary production in this coastal ecosystem.
2. Methodology
2.1. Observations
Between March 2012 and December 2019, a total of 15 oceanographic surveys were conducted at Station 30 (42°16.2′ N, 140°36.0′ E; 96 m depth) in the central part of Funka Bay. These surveys were carried out with the training vessel Ushio Maru of the Faculty of Fisheries, Hokkaido University (Figure 1). Vertical profiles of temperature, salinity and density were obtained using a Sea-Bird SBE 9plus CTD system (Sea-Bird Electronics, Bellevue, Washington, DC, USA). Seawater samples were collected using a 2.5 L Niskin water sampler at depths of 5, 10, 20, 30, 40, 50, 60, 65, 70, 75, 80 and 85 m. An additional sample was obtained at 90 m—approximately 1 m above the seafloor—using a Van Dorn water sampler. All water samples were analyzed for chlorophyll a and nutrient concentrations.
To investigate winter nutrient dynamics in Funka Bay, we selected data from the following periods for analysis: October 2012–February 2013, October 2013–February 2014, October 2014–February 2015, October 2015–February 2016 and October 2018–February 2019. The 2016–2017 winter season was excluded because observations in October, December and February were not available.
2.2. Chemical Analyses
2.2.1. Determination of Chlorophyll a Concentrations
For chlorophyll a analysis, 100 mL of seawater was filtered through a Whatman GF/F glass-fiber filter (25 mm diameter). The filter was placed in an 8 mL polypropylene tube (Sarstedt K.K., Tokyo, Japan) containing 6 mL of N,N-dimethylformamide and stored frozen in the dark at −20 °C until analysis. Before measurement, samples were thawed to room temperature and thoroughly mixed. Fluorescence was measured using a Turner Designs 10-AU fluorometer (Turner Designs, San Jose, CA, USA), and chlorophyll a concentrations were determined from a calibration curve prepared with chlorophyll a standard solutions.
2.2.2. Nutrient Concentration Measurements
Nutrient analyses were conducted on seawater collected directly from the 2.5 L Niskin bottles into 10 mL Spitz tubes containing 8 mL of sample. The tubes were stored in the dark at −20 °C until analysis and were thawed at room temperature (approximately 20 °C) immediately before measurement. Concentrations of nitrate + nitrite (NO3 + NO2), nitrite (NO2), phosphate (PO4) and silicic acid (Si(OH)4) were determined colorimetrically using a QuAAtro 2-HR autoanalyzer (BL TEC K.K., Osaka, Japan) following standard seawater methods and manufacturer’s protocols.
Calibration standards were freshly prepared prior to each analytical run. A mixed stock solution was made by diluting commercial standard solutions of nitrate-nitrogen (1.00 mg N L−1), nitrite-nitrogen (1.00 mg N L−1), phosphate-phosphorus (1.00 mg P L−1) and dissolved silica (1.00 mg Si L−1). Analytical precision and detection limits were comparable to those reported for the QuAAtro 2-HR system and sufficient to resolve the seasonal and interannual variations discussed in this study.
2.3. Depth-Integrated and Depth-Averaged Properties and Water Mass Mixing Calculations
To compare hydrographic and biogeochemical conditions among sampling dates and years, we calculated depth-integrated and depth-averaged properties for the water column in Funka Bay. In this study, the “water column” was defined as the depth range from the surface to 95 m, which corresponds to the maximum depth covered by the CTD and water-sampling casts at Station 30 (Figure 1).
Depth-integrated concentrations of nutrients and chlorophyll a (IC, units: μmol m−2 or μg m−2) were obtained from the discrete bottle data using the trapezoidal rule:
where Ci is the concentration at depth Zi and (Zi+1 − Zi) is the thickness of each depth interval. Depth-averaged concentrations ([C], units: μmol m−3 or μg m−3) were then calculated by dividing IC by the total depth of integration:
where H is the depth of the water column (H = 95 m). The same approach was applied to temperature, salinity and density profiles to obtain depth-averaged values. These depth-averaged properties will be shown in Section 3.3 and in the comparison between observed and expected wintertime nutrient concentrations.
To quantify the contribution of Oyashio water to Funka Bay in February, we estimated the mixing ratio of Oyashio water (rO) using a salinity mixing approach [14]:
where SO is the salinity of the Oyashio, SDec is the observed depth-averaged salinity of the Funka bay water in December, and SFeb is the observed depth-averaged salinity in February. We used salinity data (Table 1) from St. A01 and St. A02 along the A-line in late January (2013–2019) as the Oyashio, which provides a range of rO values.
Table 1.
Surface salinity and nutrient concentration of St. A01, St. A02 from 2013 to 2019, and St. 6 in 2023.
2.4. Oyashio Data from the A Line Monitoring
The Fisheries Research Agency of Japan established the hydrographic observation line, named “A-line” in 1987, which is the Oyashio crossing NW-to-SE line bounded by Hokkaido. The name “A-line” originates from Akkeshi, the nearest town to the first station of the line (https://ocean.fra.go.jp/a-line/a-line_index.html; accessed on 7 February 2026).
Surface salinity and nutrient concentrations at stations St. A01 and St. A02 showed relatively consistent ranges during winter observations (Table 2): salinity 32.06–32.79, Si(OH)4 21.00–27.76 μmol L−1, PO4 1.09–1.35 μmol L−1, and NO3 + NO2 10.79–13.90 μmol L−1. In addition, surface salinity and nutrient concentrations observed in February 2023 at the coastal station St.6 in Hidaka Bay (Table 1) were close to, or within, these ranges. Therefore, we used the ranges derived from St. A01 and St. A02 as the reference criteria for Oyashio water in this study.
Table 2.
Averaged air temperature from October to February of all observation years.
3. Results and Discussion
3.1. Water-Mass Structure from Fall to Winter Across All Observation Years
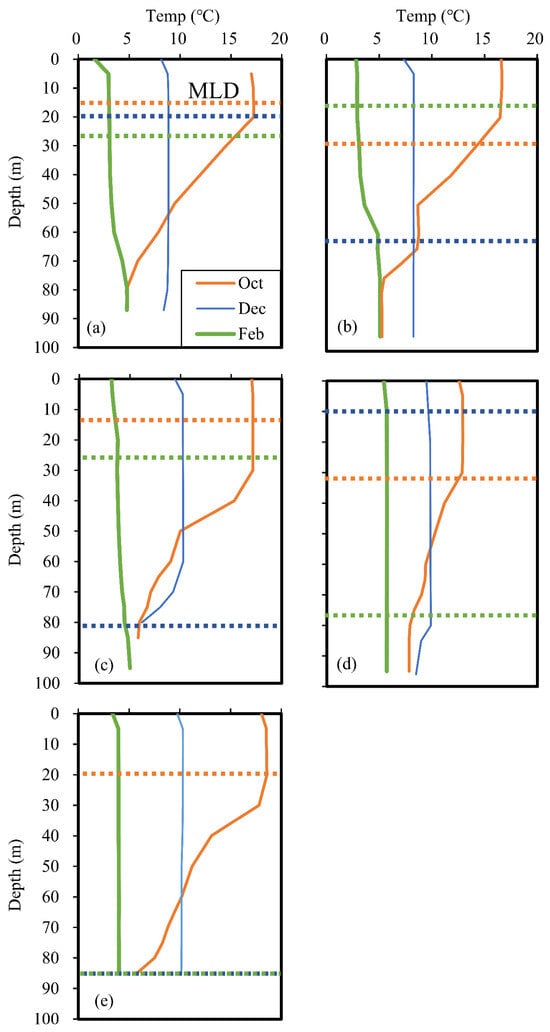
We used CTD profiling to determine the vertical distributions of water temperature and salinity in October, December, and February from October 2012 to February 2019 (Figure 2 and Figure 3). Figure 4 illustrates the temporal evolution of vertical water-mass structure based on the water-mass classification scheme specific to Funka Bay, following the definitions of [1]. Water masses in Funka Bay are classified as follows:
Figure 2.
Vertical distribution of water temperature in Funka Bay, Japan, from October to February for 2012–2019: (a) 2012–2013, (b) 2013–2014, (c) 2014–2015, (d) 2015–2016, and (e) 2018–2019. Profiles illustrate seasonal thermal structure across observation years based on CTD measurements. The mixed layer depth (MLD) is indicated by the dashed lines.
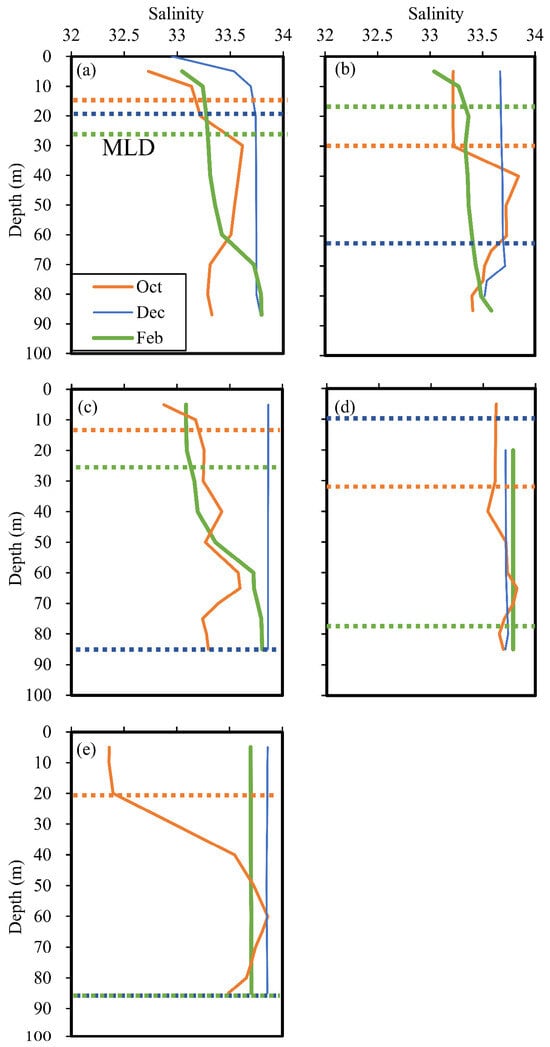
Figure 3.
Vertical distribution of salinity in Funka Bay, Japan, from October to February for 2012–2019: (a) 2012–2013, (b) 2013–2014, (c) 2014–2015, (d) 2015–2016, and (e) 2018–2019. Profiles illustrate seasonal thermal structure across observation years based on CTD measurements. The mixed layer depth (MLD) is indicated by the dashed lines.
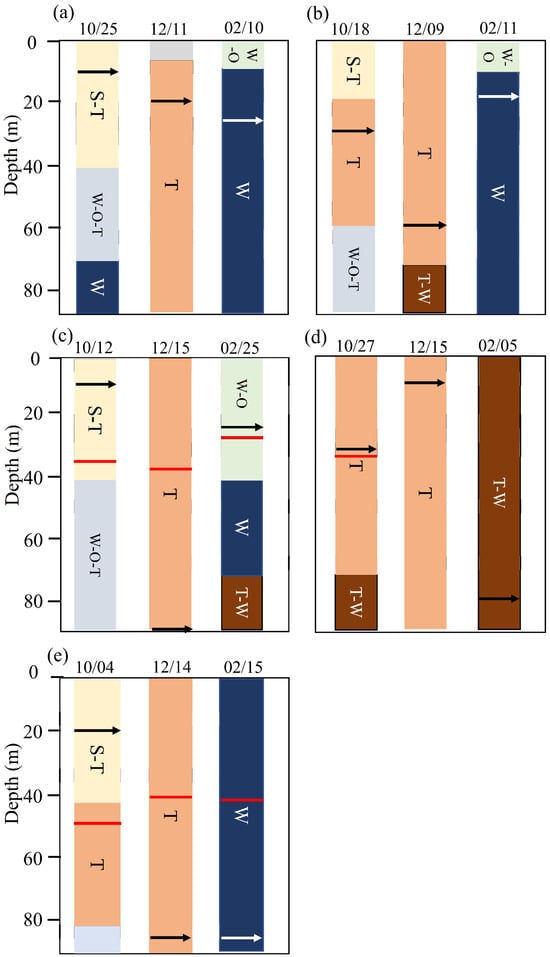
Figure 4.
Time-series changes in vertical water-mass structure of all observation years. in Funka Bay, Japan. (a) 2012–2013, (b) 2013–2014, (c) 2014–2015, (d) 2015–2016, (e) 2018–2019). Water-mass classifications are based on temperature-salinity criteria following [1,7]. O, Oyashio water; S, summer surface water; T, Tsugaru warm water; W, winter Funka Bay water. T–W, S–T, W–O, and W–O–T are transitional water types. Arrows indicate the mixed layer depth (MLD); red lines indicate the euphotic zone depth (EZD).
- Oyashio water (O): −1 to 4 °C, salinity 32.6–33.1
- Summer surface water (S): 10–25 °C, salinity 30.0–32.5
- Tsugaru warm water (T): 5–15 °C, salinity 33.5–34.2
- Winter Funka Bay water (W): −1 to 5 °C, salinity 33.25–34.2
Water masses not fitting these primary categories were further classified by [7] into transitional types:
- S–T: Mixture of summer surface water and Tsugaru warm water
- W–O–T: Winter Funka Bay water mixed with Oyashio and Tsugaru warm water
- T–W: Tsugaru warm water transitioning into winter Funka Bay water
- W–O: Winter Funka Bay water mixed with Oyashio water
Following the methodology of [15], the mixed layer depth (MLD) in this study was defined as the depth where the potential density increased by 0.03 σ (equivalent to 0.03 kg m−3). This 0.03 kg m−3 criterion was specifically selected for winter conditions, as it avoids diurnal surface variability and more accurately resolves the weakly stratified mixed layer compared to a larger threshold (0.125 kg m−3).
In October, salinity in the surface mixed layer was generally high and temperatures ranged from 9 to 15 °C, consistent with S–T conditions (a mixture of Summer Surface Water and Tsugaru warm water). At depths greater than 40 m, salinity (33.30–33.50) and temperatures (5.0–10.0 °C) indicate Tsugaru-influenced transitional conditions near the lower-salinity end of the T range, suggesting that Tsugaru Warm Current water entered Funka Bay at mid-depths (40–60 m). This type of mid-layer Tsugaru intrusion during late summer to early autumn has been reported as a recurring feature in Funka Bay [7].
Typically, in October, Tsugaru Warm Current water is observed mainly below 20 m. However, in October 2015, an anomalous structure was observed, with Tsugaru-related high-salinity water extending from the surface to 70 m. This event was likely associated with a pronounced Tsugaru inflow in October 2015 [6] together with enhanced vertical mixing under relatively low air temperatures (the minimum air temperature was 9.7 °C; Table 2) and the relatively late sampling date (27 October).
By December, the Tsugaru Warm Current water generally extended from the surface to 95 m, and salinity was relatively high across most of the water column, indicating strong Tsugaru influence during early winter. This seasonal shift was primarily driven by atmospheric forcing. The combination of low air temperature (e.g., December 2014 (−2.6) °C) and intensified monthly mean wind speeds (e.g., December 2014 (7.3) m/s; Table 2) during December triggered strong convective mixing.
In February 2013, 2014, and 2015, salinity in the upper ~40 m was generally low (often < 33.25) and temperatures ranged from 3.0 to 5.0 °C. These values were notably lower than the surface salinity observed in December of the same years, suggesting that low-salinity Oyashio water intruded into the surface layer between December and February. During this period, total precipitation over the bay area (2485 km2) ranged from 49 to 72 mm (Data is from Japan Meteorological Agency; https://www.jma.go.jp/jma/index.html; accessed on 15 September 2025). The associated freshwater input would reduce salinity by only 0.2%, which is insufficient to account for the observed decline. In addition, river-derived freshwater is likely to remain along the coastal boundary and not intrude into the bay center [16]. Therefore, the decrease in surface salinity is primarily attributed to the intrusion of low-salinity seawater from offshore—Oyashio water.
In contrast, February 2016 exhibited vertically homogeneous, high salinity (33.70), significantly higher than the February averages for 2013–2015 (33.37–33.43). The mean salinity in December 2015 (33.71) was nearly identical to that in February 2016, suggesting little or no Oyashio inflow during this period. This interpretation is consistent with [6], who reported that Oyashio water typically entered Funka Bay by the end of February between 2010 and 2014, but was absent by February 2016.
In February 2019, temperatures and salinity (2–5 °C; 33.25–34.00) were consistent with Winter Funka Bay water (W). Although the water column was largely vertically mixed, the average salinity decreased from 33.85 in December to 33.70 in February. This suggests that Oyashio water likely began intruding into the bay in early February and was subsequently redistributed by winter mixing before the February observations, such that a distinct low-salinity surface signal was not evident in February 2019.
3.2. Chlorophyll a Concentrations
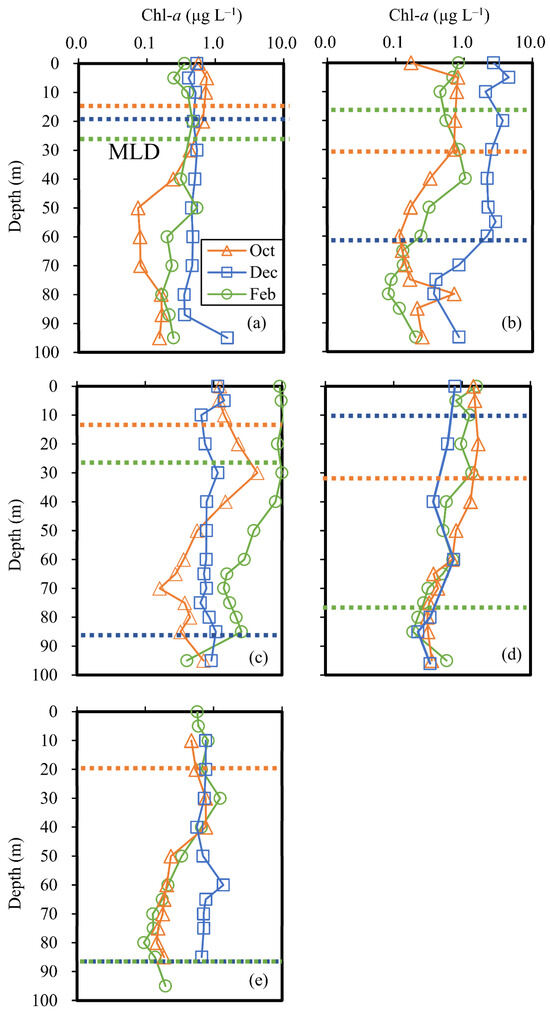
Vertical profiles of chlorophyll a from October 2012 to February 2019 are shown in Figure 5. Rather than describing each survey in detail, we focus here on the common seasonal patterns and the most notable interannual differences.
Figure 5.
Vertical distribution of chlorophyll-a concentrations from October to February (2012–2019): in Funka Bay, Japan: (a) 2012–2013, (b) 2013–2014, (c) 2014–2015, (d) 2015–2016, and (e) 2018–2019. The mixed layer depth (MLD) is indicated by the dashed lines.
In October, chlorophyll a was generally elevated within the surface mixed layer and decreased with depth, reflecting autumn phytoplankton activity under stratified conditions. Surface-layer concentrations were typically on the order of 0.2–4 μg L−1, and subsurface maxima at 10–40 m were observed in some years. Below this upper layer, chlorophyll a generally declined to low values (commonly < 0.5 μg L−1). These features are consistent with the development of an autumn bloom [7,8,9] and the occurrence of a subsurface chlorophyll maximum associated with the seasonal pycnocline.
In December, chlorophyll a exhibited two contrasting states among the observation years. In 2013, chlorophyll a remained relatively high in the upper layer (approximately 0–60 m), with values frequently exceeding 2 μg L−1 and reaching maxima > 4 μg L−1, suggesting that elevated phytoplankton biomass persisted into early winter. In 2012 and 2015, chlorophyll a was consistently low (generally < ~1.5 μg L−1) throughout the water column, indicating that the autumn bloom had already declined and that phytoplankton biomass during early winter was modest.
In February, chlorophyll a was generally low throughout the water column in most winters, with values typically <2 μg L−1, implying limited phytoplankton biomass during mid-winter when mixing is strongest. February 2015 was an exception: chlorophyll a in the upper 40 m increased markedly, reaching 8.0–10.6 μg L−1, and elevated values extended to greater depths.
3.3. Nutrient Concentrations
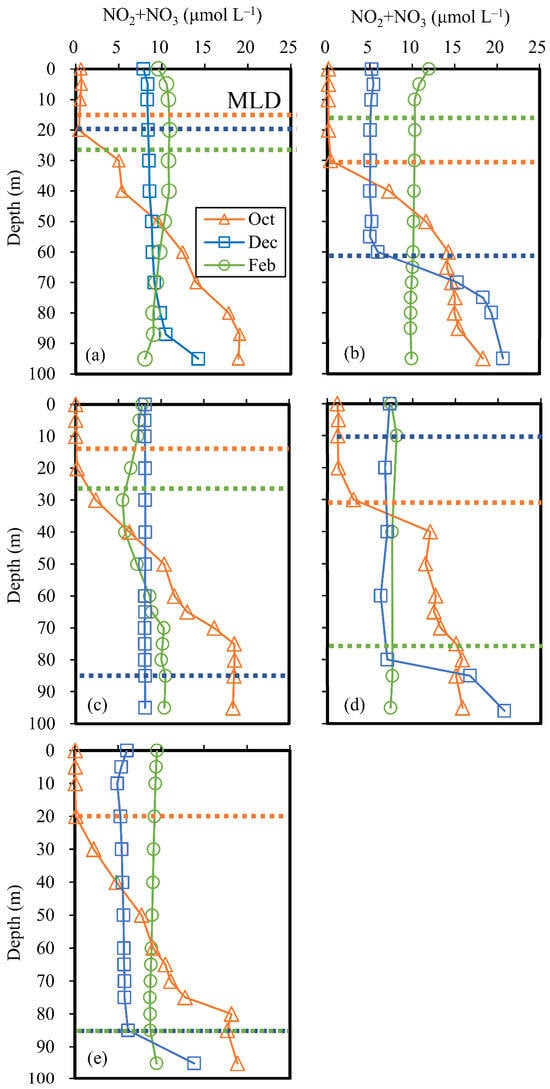
The vertical distributions of nitrate, phosphate, and silicate from 2012 to 2019 are shown in Figure 6, Figure 7 and Figure 8, respectively. Depth-integrated averages of water temperature, salinity, density, and nutrient concentrations are summarized in Table 3.
Figure 6.
Vertical distribution of nitrate and nitrite concentrations from October to February (2012–2019) in Funka Bay, Japan: (a) 2012–2013, (b) 2013–2014, (c) 2014–2015, (d) 2015–2016, and (e) 2018–2019. The mixed layer depth (MLD) is indicated by the dashed lines.
Figure 7.
Vertical distribution of phosphate concentrations from October to February (2012–2019) in Funka Bay, Japan: (a) 2012–2013, (b) 2013–2014, (c) 2014–2015, (d) 2015–2016, and (e) 2018–2019. The mixed layer depth (MLD) is indicated by the dashed lines.
Figure 8.
Vertical distribution of silicate concentrations from October to February (2012–2019) in Funka Bay, Japan: (a) 2012–2013, (b) 2013–2014, (c) 2014–2015, (d) 2015–2016, and (e) 2018–2019. The mixed layer depth (MLD) is indicated by the dashed lines.
Table 3.
Mixed layer depth (MLD); euphotic zone depth (EZD); depth averaged (with standard deviations) values of water temperature, salinity, and nutrient concentrations of all observation years.
3.3.1. Seasonal Evolution of Nutrient Distributions from October to February Across Observation Years
Across the observation years, nitrate (NO3 + NO2), phosphate (PO4), and silicate (Si(OH)4) displayed a consistent seasonal transition from a strongly stratified structure in October to a more vertically homogeneous structure by February (Figure 6, Figure 7 and Figure 8). In October, nutrient concentrations in the upper layer were generally low, while deeper waters were nutrient-rich, resulting in steep vertical gradients. For full-depth bottle profiles (maximum sampling depth ≥ 90 m), surface-layer (0–20 m) concentrations ranged from 0.05 to 1.30 µmol L−1 for NO3 + NO2, 0.05 to 0.46 µmol L−1 for PO4, and 1.80 to 3.90 µmol L−1 for Si(OH)4, whereas deep-layer (70–96 m) concentrations were substantially higher (11.12–19.06 µmol L−1, 0.96–2.27 µmol L−1, and 21.53–81.51 µmol L−1, respectively), indicating strong nutrient accumulation at depth under weak vertical mixing.
By December, vertical mixing had intensified and nutrient gradients were reduced relative to October, yielding a more uniform distribution through much of the water column. In the surface layer (0–20 m), concentrations increased to 4.92–8.42 µmol L−1 (NO2 + NO3), 0.38–0.83 µmol L−1 (PO4), and 8.92–18.80 µmol L−1 (Si(OH)4). Deep-layer concentrations in December spanned 5.76–20.74 µmol L−1 (NO3 + NO2), 0.45–2.44 µmol L−1 (PO4), and 10.61–60.48 µmol L−1 (Si(OH)4), suggesting that although mixing reduced stratification, bottom-enhanced nutrients could still persist.
By February, nutrient profiles became markedly more homogeneous, consistent with strong winter mixing. Surface-layer (0–20 m) concentrations ranged from 6.46 to 11.96 µmol L−1 (NO3 + NO2), 0.79 to 1.02 µmol L−1 (PO4), and 15.82 to 25.61 µmol L−1 (Si(OH)4), while deep-layer (70–96 m) concentrations were 7.41–10.52 µmol L−1, 0.72–1.83 µmol L−1, and 16.19–35.77 µmol L−1, respectively. Overall, the October–February evolution indicates a shift from strong stratification and low surface nutrients in autumn to a well-mixed winter structure with elevated nutrient concentrations throughout the water column.
February 2015 shows a distinct nutrient structure compared with other winters and is therefore described separately in Section 3.3.2.
3.3.2. Nutrient Concentrations in February 2015
Nutrient concentrations in February 2015 followed a different pattern than in other observation years. Nitrate concentrations in the surface layer (0–50 m) were relatively low, ranging from 5.49 to 7.78 µmol L−1. These values represent a decrease of 0.36 to 2.65 µmol L−1 compared to concentrations in December of the previous year. Nitrate levels vertically increased below 50 m, particularly from 70 m to the bottom (96 m). Phosphate and silicate exhibited similar vertical patterns. Phosphate concentrations ranged from 0.70 to 0.87 µmol L−1 in the surface layer and increased with depth; the depth-averaged concentration is 0.98 µmol L−1. Silicate concentrations were 14.27 to 18.34 µmol L−1 at 0–50 m, increasing below 70 m, with an average concentration of 23.45 µmol L−1 across all depths.
Notably, 2015 was the only observation year in which nutrient concentrations in the surface layer declined in February. Although October 2015 was cold, the preceding February was relatively warm. Air temperature was relatively mild (1.5~3.4 °C higher than other years) in February 2015 compared with other years in February (Table 2). Such mild winter conditions may have led to earlier stratification and, consequently, an earlier phytoplankton bloom, as chl-a concentrations were particularly high during this period, ranging from 3.87 to 10.55 µg L−1.
3.4. Comparison of Fall-to-Winter Nutrient Variations Across Observation Years
The depth-averaged changes in nutrient concentrations from October to December and from December to February are summarized in Table 4. Across the observation years, nutrients generally declined from October to December, indicating a net drawdown during late autumn. This seasonal decrease is consistent with biological consumption associated with autumn phytoplankton bloom [9,10,11], although in this study, the absence of observations in November prevents us from resolving the precise timing of nutrient drawdown within the October–December interval.
Table 4.
Changes in nutrient concentrations from October to December and from December to February of all observation years.
In contrast, nutrient concentrations showed a consistent tendency to increase from December to February among the observation years, except for December 2015 to February 2016. This wintertime increase implies a shift toward net replenishment of the water-column nutrient inventory, which is likely supported by a lateral exchange with Oyashio water. In Funka Bay, Oyashio water intrusion is reflected by a decrease in salinity between December and February, and the proportion of Oyashio in February varies substantially among years, indicating that the magnitude of Oyashio influence is highly variable. Oyashio inflow will be discussed in Section 3.5.
3.5. Factors Determining Changes in Nutrient Concentrations from December to February
Observational data indicate a decrease in salinity from December to February across all years (except 2016). This section discusses the mechanisms influencing nutrient concentrations during this period, with a focus on the contributions from Oyashio water inflow.
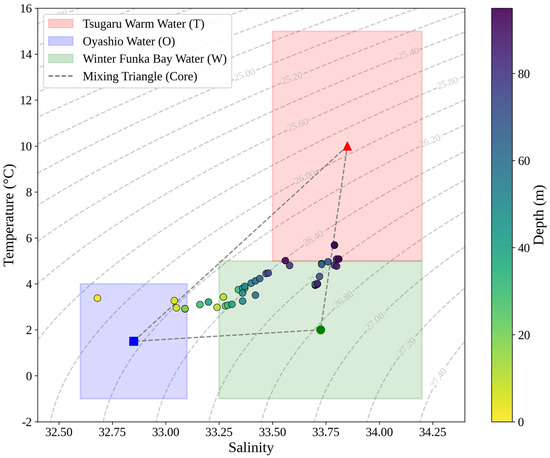
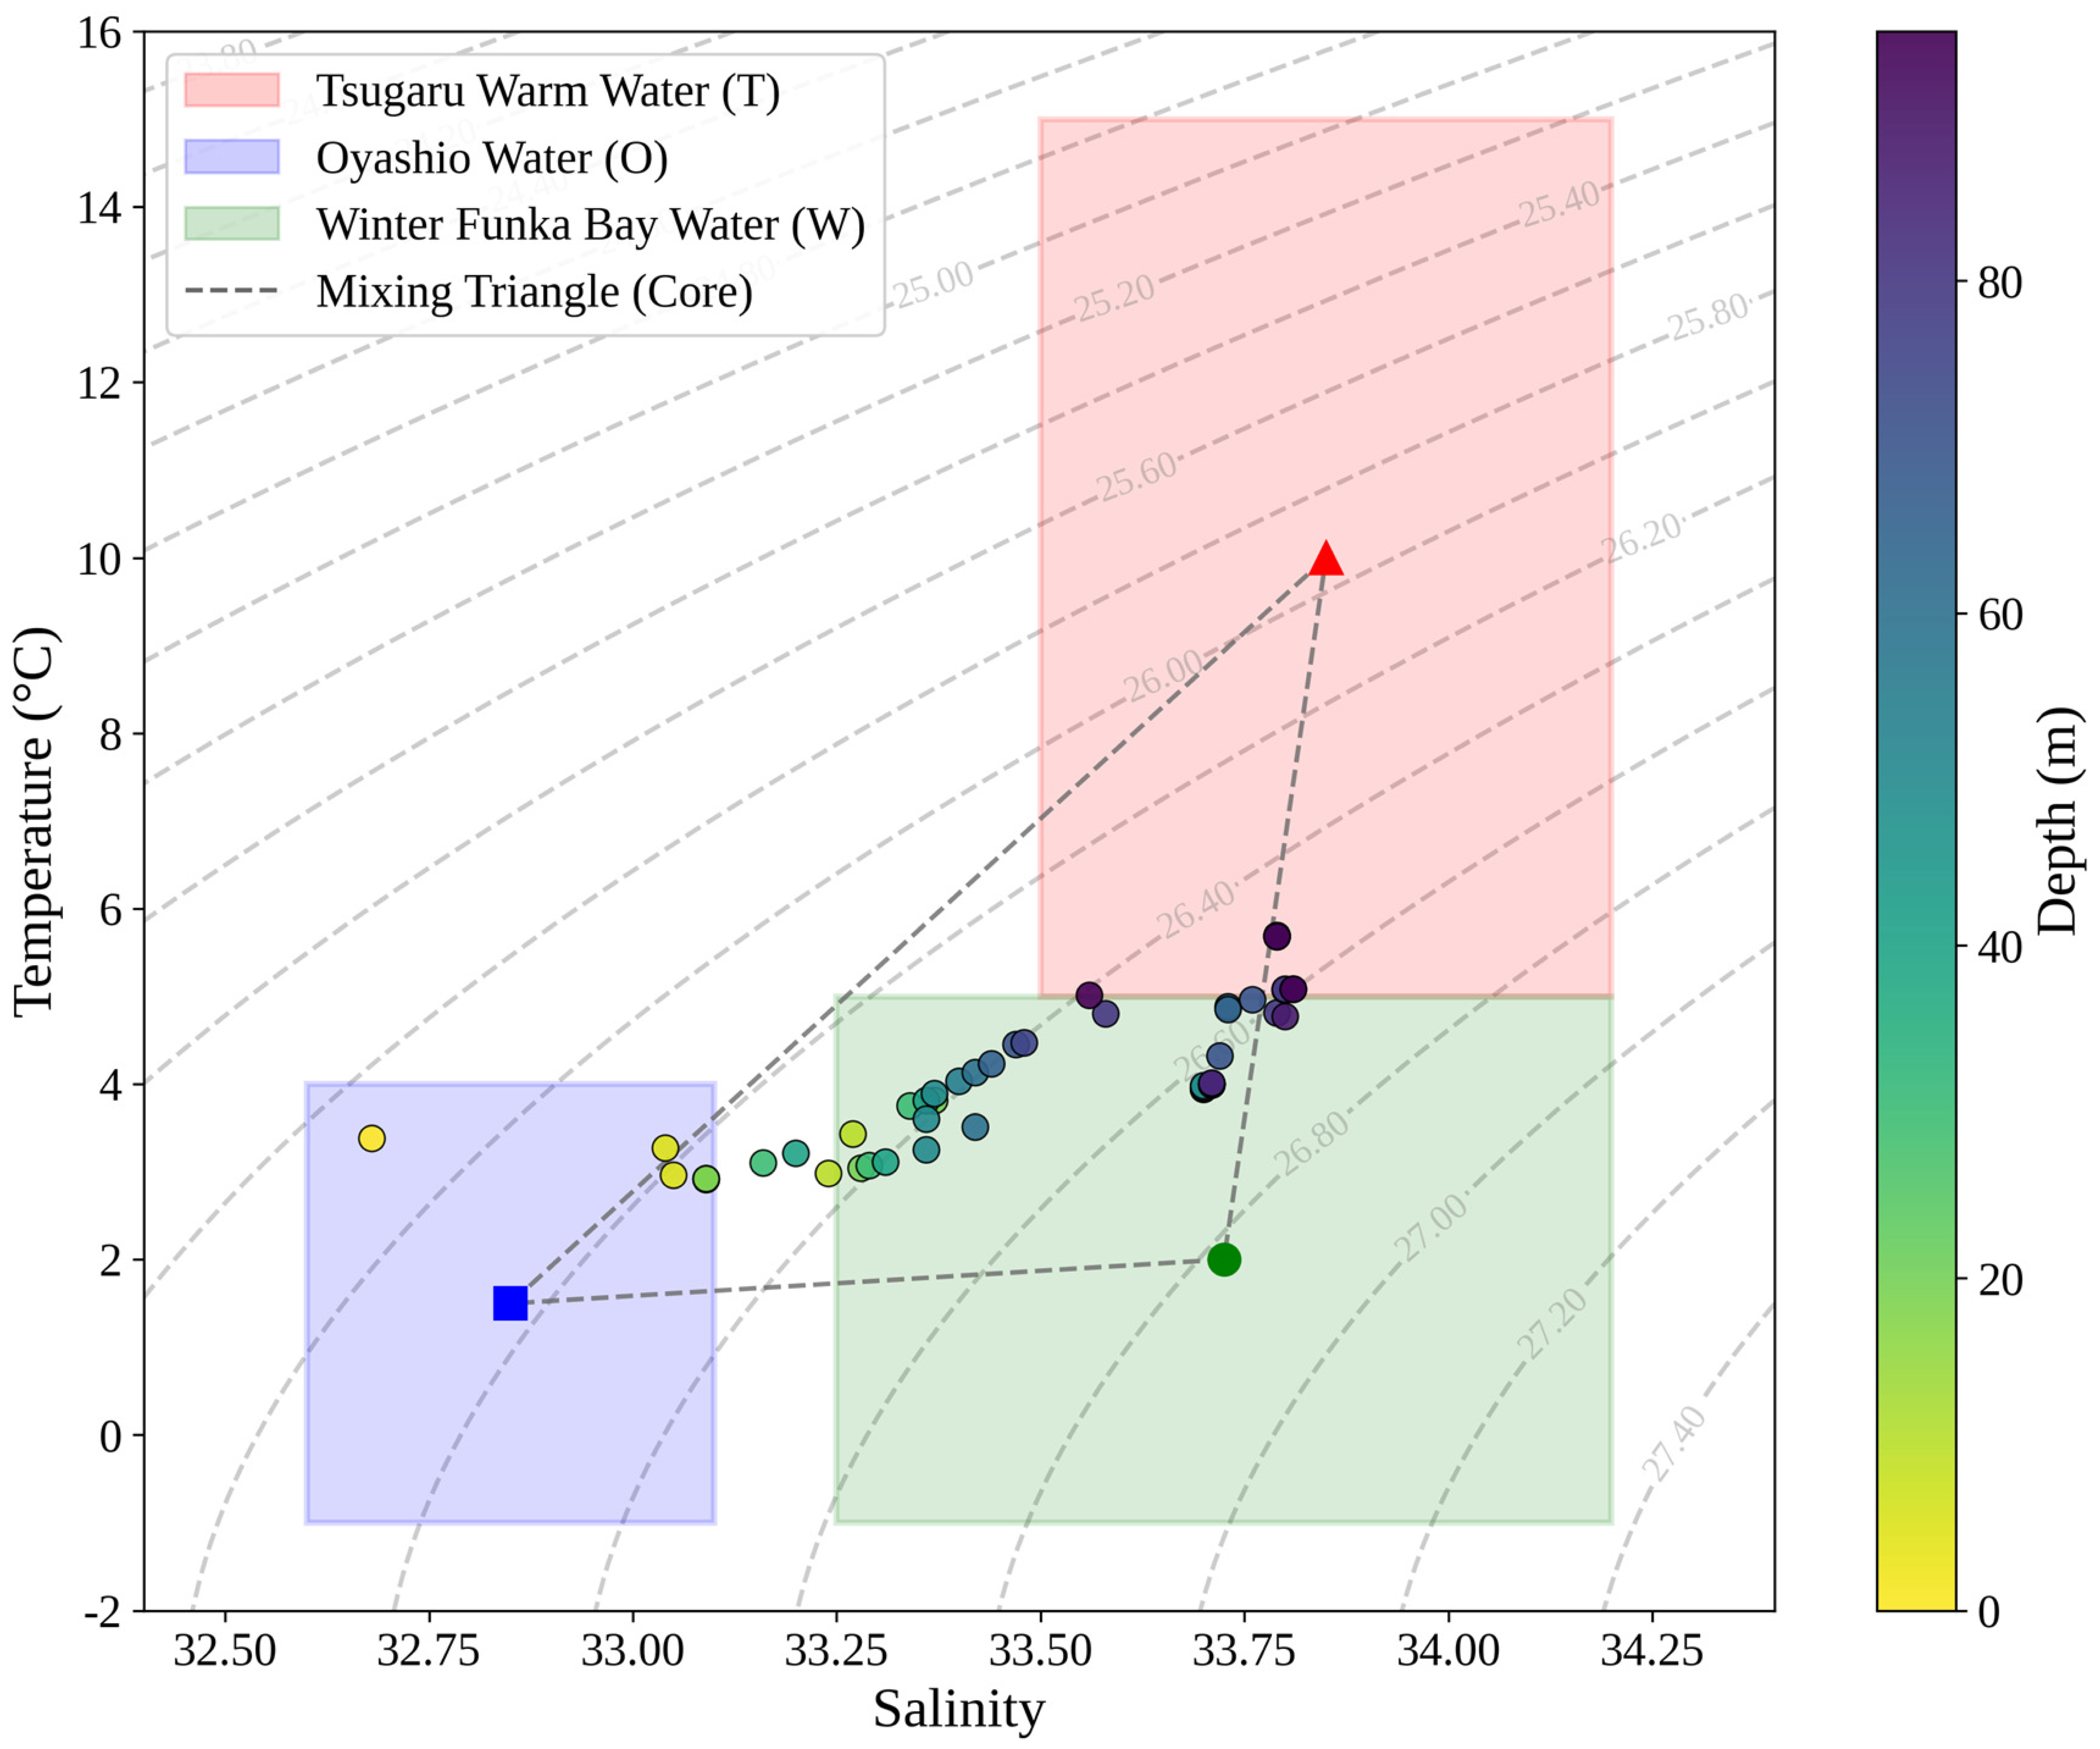
To understand the physical mixing processes controlling the bay during winter, a three-end-member temperature-salinity (T-S) mixing model was constructed for February (Figure 9). The potential water sources are defined by their characteristic temperature and salinity ranges: Tsugaru warm water (T), Oyashio water (O), and Winter Funka Bay water (W). As illustrated in Figure 9, the observed February water samples (scatter points) predominantly fall along the mixing line between the Oyashio water (O) and the Winter Funka Bay water (W), with a significant portion clustering tightly within the W end-member box. Notably, the depth-resolved data reveals that the colder and relatively fresher surface/subsurface waters are strongly influenced by the Oyashio intrusion, while the deeper waters maintain the characteristics of the locally formed Winter Funka Bay water.
Figure 9.
Temperature-salinity (T-S) diagram with potential density anomalies (dashed grey contours) for February observation data. The scatter points represent the observed bottle data, colored by depth. Three distinct water mass end-members are indicated by shaded rectangular boxes, reflecting their natural variability: Tsugaru warm water (T, red), Oyashio water (O, blue), and Winter Funka Bay water (W, green).
To quantify the contribution of Oyashio water to Funka Bay in February, we estimated the mixing ratio of Oyashio water (rO) using a salinity mixing approach (Section 2.2.1).
Based on this calculation, the Oyashio water proportion in February was 21.0–21.1% (2013), 18.6–33.3% (2014), 33.1–43.4% (2015), 0% (2016), and 12.8–12.9% (2019) (Table 5). The absence of Oyashio water in February 2016 (rO ≈ 0) indicates that wintertime hydrographic and biogeochemical conditions in Funka Bay can vary substantially depending on the occurrence and magnitude of Oyashio water intrusion.
Table 5.
Proportion of Oyashio water in February.
In addition to supply by Oyashio intrusion, winter nutrients in Funka Bay can be modified by biological uptake and internal recycling. Funka Bay commonly experiences an autumn phytoplankton bloom [9], and the elevated chl-a observed in October–December in this study suggests that a portion of nutrients consumed during autumn can be regenerated through decomposition of organic matter on seasonal time scales [11].
To evaluate whether the February nutrient concentrations can be explained by conservative mixing alone, we estimated the expected February nutrient concentrations ([Nuts]) from a two-endmember mixing model:
where NutO and NutDec are the nutrient concentrations in the Oyashio endmember and in Funka Bay water in December, respectively, and rO is the Oyashio proportion from Equation (3). ΔNutOct-Dec, accounts for the net nutrient drawdown observed from October to December and is introduced here as a regeneration correction under the assumption that nutrients consumed during the autumn bloom are fully regenerated during the subsequent winter period (December–February) and are then redistributed throughout the water column by winter mixing. Accordingly, ΔNutOct-Dec is defined as the depth-averaged change between October and December (Table 4), such that a negative October–December change (net drawdown by autumn uptake) contributes a positive correction to the expected February concentration when complete wintertime regeneration is assumed. Using St. A01 and St. A02 as alternative Oyashio endmembers yields a range of [Nut] values (Table 6).
Table 6.
Expected and observed nutrient concentration in February of all Observation years.
Comparison between the expected and observed February concentrations indicates that the conservative two-endmember mixing model reproduces the February nutrient concentrations reasonably well for most winters (Table 6). For example, observed NO3 + NO2 concentrations are close to the mixing-based estimates in 2013 (10.04 vs. 10.22–10.24 μmol L−1), 2014 (10.11 vs. 9.80–10.83 μmol L−1), 2016 (7.69 vs. 8.52 μmol L−1), and 2019 (9.02 vs. 8.06–8.26 μmol L−1). Similarly, PO4 concentrations are generally comparable to the conservative-mixing estimates (e.g., 0.98 vs. 1.07 μmol L−1 in 2013; 1.03 vs. 0.95–1.01 μmol L−1 in 2014; 0.83 vs. 0.82 μmol L−1 in 2016; and 0.82 vs. 0.77–0.79 μmol L−1 in 2019). These agreements suggest that, in most winters, the December–February nutrient levels can be interpreted primarily in terms of variable Oyashio contribution and nutrients regeneration.
February 2015 is a clear exception (Table 6). In 2015, the observed February concentrations were substantially lower than the mixing-based estimates (e.g., NO3 + NO2 = 8.36 vs. 10.40–11.53 μmol L−1; PO4 = 0.98 vs. 1.13–1.20 μmol L−1; Si(OH)4 = 23.45 vs. 30.89–33.12 μmol L−1). This deviation is consistent with the onset of phytoplankton growth by late February 2015, as indicated by the unusually high Chl-a concentrations in February 2015 (Section 3.3.2). Therefore, we interpret the 2015 mismatch as reflecting a biological drawdown that had already begun by the observation date; before this drawdown, the wintertime nutrient levels would likely have been closer to the conservative-mixing estimates.
In contrast, the calculated and observed February silicate concentrations appear to differ more substantially in 2013–2015 (Table 6), and the underlying cause is not yet clear. One plausible explanation is that complete winter regeneration of the autumn-bloom silicate drawdown may not be achieved by February (with part of the biogenic silica remaining in particulate/sedimentary pools). In addition, silicate recycling may also vary with temperature because biogenic-silica dissolution accelerates as temperature increases [17] In 2012–2014 (8.78 °C, 8.79 °C, 8.26 °C) were relatively lower than those in 2015 and 2018 (9.64 °C, 9.59 °C), the rate at which silicate is regenerated from biogenic silica may have differed among winters, potentially contributing to the observed deviations between calculated and observed silicate concentrations.
In this semi-enclosed system (Funka Bay), nutrient concentrations likely decreased during autumn (October–December) due to primary production associated with the autumn phytoplankton bloom. During winter (December–February), organic matter produced during the autumn bloom was likely remineralized, returning regenerated inorganic nutrients to the water column. Accordingly, the December–February nutrient changes can largely be interpreted as the combined effects of mixing between Funka Bay water and intruding Oyashio water, together with wintertime regeneration of the autumn-bloom drawdown. However, when the spring bloom has already commenced by the time of the February survey, additional biological drawdown may be evident as lower observed nutrient concentrations. Because the present study did not resolve the autumn bloom in detail, future observations that continuously capture both the autumn and spring blooms are required.
3.6. Biogeochemical Drivers: Sediment Flux, Riverine Inputs, and Light Constraints
While physical mixing primarily drives the winter nutrient resupply, the role of internal biogeochemical cycling, particularly benthic-pelagic coupling, cannot be overlooked. Previous studies have demonstrated that nutrient flux from sediments exerts a strong control on the nitrogen distribution in Funka Bay [18]. During summer, the development of hypoxic conditions in the bottom layer facilitates the accumulation of macronutrients and dissolved iron. As the water column is reoxygenated by intense vertical mixing in winter, these benthic reservoirs are rapidly transported to the upper layers [19], significantly modifying the nutrient stoichiometry. In addition to inorganic nutrients, dissolved organic nitrogen, notably urea, is present in appreciable concentrations and likely serves as a crucial supplementary nitrogen source for the winter and spring phytoplankton communities [4].
Regarding external terrestrial sources, our initial model assumed that riverine inputs mainly impacted the near-shore regions of the bay [16]. However, recent investigations using fluorescent dissolved organic matter (FDOM) as a tracer revealed that riverine supply is a major source of freshwater to the Coastal Oyashio water (COW) [20]. This suggests a broader regional impact: the riverine supply of materials from outside Funka Bay strongly influences the chemical properties of the COW. Consequently, the “Oyashio endmember” entering the bay is already pre-conditioned by terrestrial nutrient and organic matter inputs.
Evaluating the winter nutrient drawdown requires considering light availability. During typical winter conditions, deep vertical mixing transports phytoplankton below the euphotic zone, strictly limiting photosynthetic productivity despite nutrient abundance. PAR (photosynthetically active radiation) measurements in Funka Bay confirm that light limitation is a primary control on winter/early spring biological activities [7,21].
However, the apparent productivity observed in February 2015 can be contextualized by the exceptionally mixed layer depth (26 m) during that specific period. This physical stabilization likely retained phytoplankton within the euphotic zone, alleviating light limitation and triggering an early subsurface bloom. Furthermore, it is important to note that the decline in nutrient concentrations during the deeply mixed, light-limited winter months may not solely represent photosynthetic uptake. Recent reports highlight considerable nutrient consumption in the dark by microbial communities and overwintering phytoplankton [22], which acts as a secondary sink for the winter nutrient inventory.
4. Conclusions
This study characterized the fall-to-winter evolution of water-mass structure and nutrient distributions in Funka Bay (October–December–February, 2012–2019). October was generally characterized by weak vertical mixing and strong nutrient stratification, with low nutrient concentrations in the surface mixed layer and markedly higher concentrations at depth; progressive mixing toward December reduced these vertical gradients, and by February the water column approached near-uniform nutrient distributions. Interannual variability in winter nutrient replenishment was closely linked to the occurrence and magnitude of Oyashio intrusion, quantified using A-line stations St. A01 and St. A02 as endmembers.
To evaluate whether February nutrient concentrations can be explained by conservative mixing alone, we applied a two-endmember mixing model between Oyashio water and December Funka Bay water and incorporated a regeneration correction term that assumes nutrients consumed during the October–December autumn bloom are fully regenerated during December–February and redistributed by winter mixing. Expected February nutrient concentrations were generally close to observations for most winters, indicating that winter nutrient levels can be interpreted primarily in terms of variable offshore-water contribution and seasonal regeneration. February 2015 was a clear exception, with observed nutrients markedly lower than expected; this mismatch is consistent with nutrient drawdown after the early onset of the bloom by late February, and the pre-drawdown winter concentrations were likely similar to the mixing-based expectations.
Overall, in this semi-enclosed system (Funka Bay), the late-winter nutrient state can be viewed as the outcome of autumn-bloom drawdown followed by wintertime regeneration, superimposed on variable Oyashio intrusion and winter mixing. When the spring bloom has already commenced by the February survey (as in 2015), additional biological uptake can depress the observed nutrient concentrations, underscoring the need for continuous observations spanning both the autumn and spring blooms.
Author Contributions
Methodology, A.O., H.A., K.K. and T.T.; Resources, A.O., K.K., Y.K., N.K. and T.I.; Data curation, A.O., Y.K., N.K., T.I., T.C. and K.K. Writing—review and editing, T.C.; H.A., T.T. and A.O.; Visualization, T.C.; Project administration, H.A. and A.O. Funding acquisition, A.O., H.A. and T.T. All authors have read and agreed to the published version of the manuscript.
Funding
This research was funded by the Japan Society for the Promotion of Science KAKENHI (grant numbers 16K07834, 22K19838, 23K11388 and 25450269).
Data Availability Statement
All data analyzed in this study were collected via the Hokkaido University research vessel T/S Ushio-maru from 2012 to 2019. Requests for further information should be addressed to the corresponding author.
Acknowledgments
This study was supported by Research Projects from the Hokusui Society Foundation, Sapporo, Japan, for fiscal years 2012–2019 and JSPS KAKENHI (grant numbers 16K07834, 22K19838, 23K11388 and 25450269). We thank the captain and crews of T/S Ushio-maru (Hokkaido University). All individuals mentioned in the Acknowledgements have provided their informed consent to be included.
Conflicts of Interest
The authors declare no conflicts of interest.
References
- Ohtani, K.; Kido, K. Oceanographic structure of Funka Bay. Bull. Fac. Fish. Hokkaido Univ. 1980, 31, 84–114, (In Japanese with English Abstract and Legends). [Google Scholar]
- Kudo, I.; Yoshimura, T.; Yanada, M.; Matsunaga, K. Exhaustion of nitrate terminates a phytoplankton bloom in Funka Bay, Japan: Change in SiO4:NO3 consumption rate during the bloom. Mar. Ecol. Prog. Ser. 2000, 193, 45–51. [Google Scholar] [CrossRef] [Scilit]
- Rosa, A.L.; Isoda, Y.; Uehara, K.; Aiki, T. Seasonal variations of water system distribution and flow patterns in the southern sea area of Hokkaido, Japan. J. Oceanogr. 2007, 63, 573–588. [Google Scholar] [CrossRef] [Scilit]
- Kudo, I.; Hisatoku, T.; Yoshimura, T.; Maita, Y. Primary productivity and nitrogen assimilation with identifying the contribution of urea in Funka Bay, Japan. Estuar. Coast. Shelf Sci. 2015, 158, 12–19. [Google Scholar] [CrossRef] [Scilit]
- Kuroda, H.; Toya, Y.; Shiga, N.; Watanabe, T.; Nishioka, J.; Hasegawa, D.; Taniuchi, Y.; Kuwata, A. Variation of size-fractionated Fe concentrations and Fe(III) Influence of Coastal Oyashio water on massive spring diatom blooms in the Oyashio area of the North Pacific Ocean. Prog. Oceanogr. 2019, 175, 328–344. [Google Scholar] [CrossRef] [Scilit]
- Abe, H.; Yahiro, Y.; Hasegawa, T.; Hirawake, T.; Onishi, H.; Ooki, A.; Takatsu, T.; Sasaki, K.; Wakita, M.; Kaneko, H.; et al. Intrusion of Coastal Oyashio Water to Funka Bay and Tsugaru Strait occasionally disturbed by Kuroshio-originating warm core ring. J. Oceanogr. 2023, 79, 349–366. [Google Scholar] [CrossRef] [Scilit]
- Ooki, A.; Shida, R.; Otsu, M.; Onishi, H.; Kobayashi, N.; Iida, T.; Nomura, D.; Suzuki, K.; Yamaoka, H.; Takatsu, T. Isoprene production in seawater of Funka Bay, Hokkaido, Japan. J. Oceanogr. 2019, 75, 485–501. [Google Scholar] [CrossRef] [Scilit]
- Miki, C.; Abe, H.; Onishi, H.; Ooki, A.; Takatsu, T. Multi-month prediction of summertime hypoxia occurrence in the bottom of Funka Bay, Japan, with a focus on the wintertime surface heat flux. J. Mar. Syst. 2025, 247, 104035. [Google Scholar] [CrossRef] [Scilit]
- Maita, Y.; Odate, T. Seasonal Changes in Size-Fractionated Primary Production and Nutrient Concentrations in the Temperate Neritic Water of Funka Bay, Japan. J. Oceanogr. Soc. Jpn. 1988, 44, 268–279. [Google Scholar] [CrossRef] [Scilit]
- Kuma, K.; Katsumoto, A.; Shiga, N.; Sawabe, T.; Matsunaga, K. Variation of size-fractionated Fe concentrations and Fe (III) hydroxide solubilities during a spring phytoplankton bloom in Funka Bay Japan. Mar. Chem. 2000, 71, 111–123. [Google Scholar] [CrossRef] [Scilit]
- Sasaki, H.; Miyamura, T.; Saitoh, S.; Ishizaka, J. Seasonal variation of absorption by particles and colored dissolved organic matter (CDOM) in Funka Bay, southwestern Hokkaido, Japan. Estuar. Coast. Shelf Sci. 2005, 64, 447–458. [Google Scholar] [CrossRef] [Scilit]
- Cloern, E.J.; Foster, Q.S.; Kleckner, A.E. Phytoplankton primary production in the world’s estuarine-coastal ecosystems. Biogeosciences 2014, 11, 2477–2501. [Google Scholar] [CrossRef] [Scilit]
- Kudo, I.; Yoshimura, T.; Lee, C.-W.; Yanada, M.; Maita, Y. Nutrient regeneration at bottom after a massive spring bloom in a subarctic coastal environment, Funka Bay, Japan. J. Oceanogr. 2007, 63, 791–801. [Google Scholar] [CrossRef] [Scilit]
- Sugie, K.; Kuma, K.; Fujita, S.; Nakayama, Y.; Ikeda, T. Nutrient and diatom dynamics in the region of the western subarctic Pacific Ocean. Deep-Sea Res. Part II Top. Stud. Oceanogr. 2010, 57, 447–458. [Google Scholar] [CrossRef] [Scilit]
- Montegut, C.B.; Madec, G.; Fischer, A.S.; Tada, Y.; Lazar, A.; Iudicone, D. Mixed layer depth over the global ocean: An examination of profile data and a profile-based climatology. J. Geophys. Res. Ocean. 2004, 109, 12. [Google Scholar]
- Nakada, S.; Baba, K.; Sato, M.; Natsuike, M.; Ishikawa, Y.; Awaji, T.; Koyamada, K.; Saitoh, S. The role of snowmelt runoff on the ocean environment and scallop production in Funka Bay, Japan. Prog. Earth Planet. Sci. 2014, 1, 25. [Google Scholar] [CrossRef] [Scilit]
- Kamatani, A. Dissolution rates of silica from diatoms decomposing at various temperatures. Mar. Biol. 1982, 68, 91–96. [Google Scholar] [CrossRef] [Scilit]
- Montani, S.; Maita, Y.; Fukase, S. Flux of nitrogen compounds in coastal marine sediment and pore water (Funka Bay, Hokkaido). Chem. Geol. 1980, 30, 35–45. [Google Scholar] [CrossRef] [Scilit]
- Hioki, N.; Kuma, K.; Morita, Y.; Miura, D.; Ooki, A.; Tanaka, S.; Onishi, H.; Takatsu, T.; Kobayashi, N.; Kamei, Y. Regeneration dynamics of iron and nutrients from bay sediment into bottom water of Funka Bay, Japan. J. Oceanogr. 2015, 71, 703–714. [Google Scholar] [CrossRef] [Scilit]
- Mizuno, Y.; Nishioka, J.; Tanaka, T.; Tada, Y.; Suzuki, K.; Tsuzuki, Y.; Sugimoto, A.; Yamashita, Y. Determination of the freshwater origin of Coastal Oyashio Water using humic-like fluorescence in dissolved organic matter. J. Oceanogr. 2018, 74, 509–521. [Google Scholar] [CrossRef] [Scilit]
- Shimizu, Y.; Ooki, A.; Ohnishi, H.; Takatsu, T.; Tanaka, S.; Inagaki, Y.; Suzuki, K.; Kobayashi, N.; Kamei, Y.; Kuma, K. Seasonal variation of volatile organic iodine compounds in the water column of Funka Bay, Hokkaido, Japan. J. Atmos. Chem. 2017, 74, 205–225. [Google Scholar] [CrossRef] [Scilit]
- Umezawa, S.; Tozawa, M.; Nosaka, Y.; Nomura, D.; Onishi, H.; Hiroto, A.; Takatsu, T.; Ooki, A. Significant nutrient consumption in the dark subsurface layer during a diatom bloom: A case study on Funka Bay, Hokkaido, Japan. Biogeosciences 2023, 20, 421–438. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.