


Abstract
Soil mulching influences soil organic carbon (SOC) dynamics and microbial communities, yet the functional potential linking these factors remains unclear. This two-year field study compared biodegradable liquid film (BLF, C:N = 26:1, 161 kg C·ha−1) and grapevine branch mulch (GBM, C:N = 51:1, 2790 kg C·ha−1) applied in-row in a vineyard, with clean tillage as control. The Vitis vinifera cv. Meili was used as the test material, SOC fractions were determined and metagenomic sequencing was performed. The results showed that GBM had the highest SOC content and significantly increased the levels of total organic carbon, all five labile fractions, and the three recalcitrant fractions. BLF significantly increased the levels of recalcitrant fractions, while its effect on labile fractions varied by year. Metagenomic analysis revealed that the two mulching treatments significantly influenced the abundances of Acidobacteria, Verrucomicrobia, and Bacteroidetes. Redundancy analysis identified soil moisture, pH, SOC, and total nitrogen as key drivers of community structure. Mulching downregulated carbon fixation and methane metabolism genes but upregulated carbohydrate metabolism pathways, including O-glycan biosynthesis, which correlated positively with SOC. Glycosyl transferases were the dominant carbohydrate-active enzymes across all treatments. These results demonstrate that GBM and BLF differentially affect SOC fractions and microbial functional traits, providing empirical evidence for mulch selection in vineyard carbon management.
1. Introduction
In the context of global climate change, the dynamics of carbon sources, sinks, and sequestration in agricultural ecosystems have become a research priority [1,2]. As important carbon sinks, vineyards store large amounts of carbon, with Cabernet Sauvignon and Chardonnay vineyards storing 42.75 t·hm−2 and 8.02 t·hm−2, respectively [3]. The stored soil organic carbon (SOC) plays a critical role in maintaining ecosystem health and function, serving as an essential source of nutrients and energy for plant growth and soil organisms [4]. To enhance the sequestration of SOC and reduce soil carbon emissions, it is necessary to elucidate the processes and regulatory mechanisms underlying SOC sequestration in vineyards, with particular attention to the role of soil microorganisms as the primary drivers of carbon turnover and stabilization.
Plant-derived organic carbon has been considered as the primary contributor to organic carbon [5], but recent studies suggest that microorganisms may be the main source of SOC [2,6], with microbial biomass contributing as much as 50–80% of SOC [7]. Soil microorganisms play a crucial role in the balance between carbon input and output in soil. They influence the synthesis, transformation, and retention of carbon in soil as decomposers, plant symbionts, or pathogens, thereby playing a key role in the carbon cycle [8,9]. During electron transport processes, soil microorganisms obtain energy through dissimilation via respiration or fermentation, thereby releasing carbon, and synthesize organic matter to assimilate or fix carbon. These processes constitute intracellular turnover [2]. Autotrophic microorganisms assimilate inorganic carbon into organic carbon through six major pathways: the pentose phosphate pathway, the tricarboxylic acid (TCA) cycle, the 3-hydroxypropionate/4-hydroxybutyrate cycle, the dicarboxylate/4-hydroxybutyrate cycle, the 3-hydroxypropionate bicycle, and the anaerobic acetyl-CoA pathway [10]. Heterotrophic microorganisms fix CO2 via assimilatory carboxylation and non-assimilatory reactions in the TCA cycle, a process known as microbial dark fixation [11]. The abundance, diversity, and community structure of soil microorganisms directly influence SOC turnover processes [12,13]. Conversely, changes in organic carbon allocation patterns and utilization efficiency feedback to shape soil microbial communities [14]. Ultimately, biotic and abiotic factors regulate microbial community structure and the soil environment through a series of transformations, bringing the carbon cycle to a state of equilibrium.
Soil management, particularly through mulching, is a critical agronomic practice that significantly influences the growth and development of fruit trees. Mulching orchard surfaces with appropriate materials helps regulate soil temperature and moisture [15], reduce soil erosion [16], enhance soil fertility [17], improve soil structure [18], and influence soil microbial communities and carbon dynamics [19,20,21,22]. Humic acid-based biodegradable liquid film (BLF) is an environmentally friendly soil structure conditioner widely used as an alternative to traditional plastic mulch to reduce environmental pollution and improve soil management efficiency [23,24]. Grapevine pruning branches (GBM) are rich in elements such as nitrogen, phosphorus, and potassium, as well as biomass energy, and are commonly used for mulching or soil incorporation, thereby promoting microbial proliferation [25]. Recent studies have advanced the understanding of how these mulching materials regulate soil microbial communities and carbon cycling. Biodegradable film mulching has been shown to enhance microbial diversity and metabolism while reducing CO2 emissions [15,26]. Orchard branch mulching similarly reduces bulk density, improves soil micro-ecological environments and enhances carbon sequestration [22,27]. However, the specific regulatory mechanisms through which these mulching practices affect soil microbial community functions and carbon cycling processes remain inadequately understood, particularly at the metagenomic level.
Therefore, this study applied BLF and GBM mulching treatments to vineyards over two years with the following objectives: (i) to determine the changes in soil organic carbon fractions under different mulching practices; (ii) to reveal the shifts in soil microbial community structure and functional genes associated with carbon cycling using metagenomic sequencing; and (iii) to explore the relationships between microbial community composition, carbon-cycle functional pathways, and organic carbon fractions. By addressing these objectives, we aim to provide a mechanistic understanding of how contrasting mulching strategies regulate soil carbon dynamics in vineyard systems.
2. Materials and Methods
2.1. Experimental Site and Materials
The experiment was conducted at the Sheng Tang Winery vineyard in Xianyang City, Shaanxi Province, located in the central Guanzhong Plain (34°27′ N, 108°8′ E). The region has the warm temperate climate of East Asia, with an altitude of 514 m, an average annual temperature of 15.12 °C, and annual rainfall of 660 mm. The soils in the vineyard exhibited a relatively uniform composition, predominantly loam.
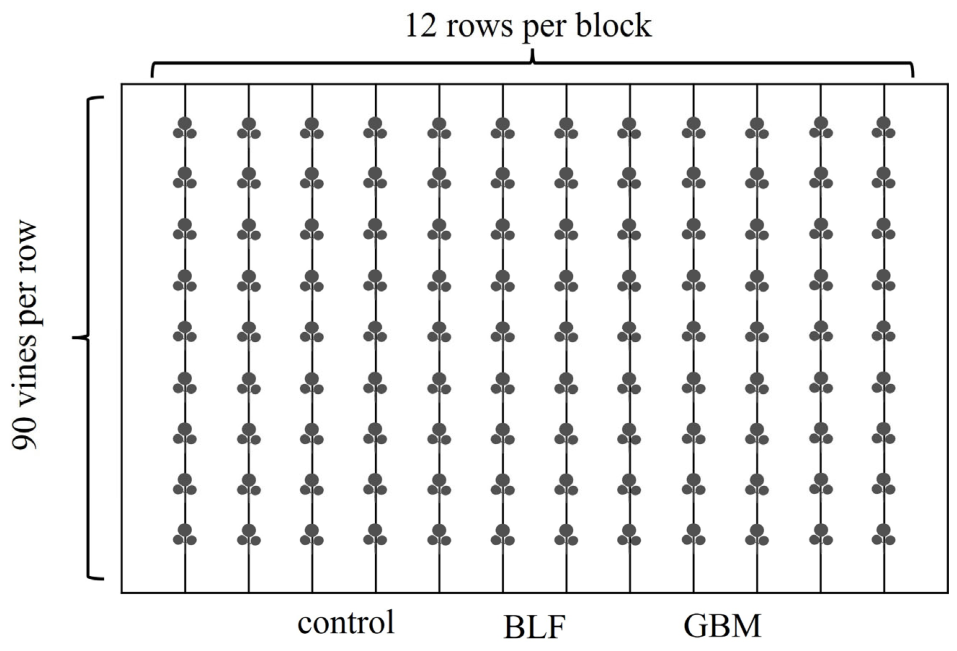
Vitis vinifera L. cv ‘Meili’, bred by the College of Enology at Northwest A&F University, was used as experimental material. The vines were planted in 2008 with a spacing of 1.0 m × 2.5 m, a row length of 90 m, trained to a single trellis with single trunk and double arms, and pruned using a combination of long and short spurs. The experimental plot was divided into three blocks with three replicates, two rows per treatment, and 90 vines per row. To avoid wind drift and edge effects, the treatments were arranged in nonadjacent rows. The treatment of each block as replicate is shown in Figure A2. For statistical analysis, the three blocks were treated as three biological replicates rather than as variable factors.
The two mulching materials selected for the experiment were a biodegradable liquid film (BLF) and one-year-old branches (GBM) obtained from winter pruning. The BLF material was independently developed by the research team and consists of a mineral matrix and humic acid macromolecules combined with suspending agents, emulsifiers, and other additives. BLF has a dry matter content of 68.7% and contains 78.0% carbon (elemental mass/dry matter mass), 3.0% nitrogen (N), 0.25% potassium (K), and 0.7% sulfur (S), with a carbon-to-nitrogen ratio of 26:1 (m/m). The BLF material was diluted with water (BLF: water = 1:10, v/v) and sprayed on the soil surface with an application rate of 300 kg·ha−1 of undiluted solution, covering a width of 50 cm. The carbon input of BLF treatment is 161 kg/ha.
The one-year-old branches used for mulching were also from the cv. ‘Meili’ and were collected during winter pruning in January. The dry matter content of the branches is 62%, contains 45.0% C (elemental mass/dry matter mass), 0.88% N, 0.75% K, 0.03% S, 0.07% phosphorus (P), 0.57% calcium (Ca), and 0.08% magnesium (Mg), with a carbon-to-nitrogen ratio of 51:1 (m/m). In March of the following year, the branches were shredded into small pieces less than 20 cm long and applied to the soil surface within the rows at a width of 50 cm and a thickness of 10 cm. The application rate of branches is 10 t/ha, resulting in a carbon input of 2790 kg/ha.
2.2. Experimental Design and Sample Collection
The experiment was conducted during the growing seasons of 2021 and 2022. Biodegradable liquid film (BLF) and shredded grape branches (GBM) were used for soil mulching, with clean tillage as the control (Figure A1). The experiment employed a one-way block design, with three biological replicates per treatment. Each replicate consisted of two rows of grapevines, with 90 plants per row. Rows adjacent to roads were avoided, and treatments were arranged in nonadjacent rows. In March of each year, before grape budding, mulching treatments were applied within the rows, while inter-rows were left with natural grass cover. Consistent cultural and water–fertilizer management practices were applied throughout the growing season across all treatments.
Topsoil (0–20 cm) samples were collected using a 4 cm soil auger following a five-point sampling method in September of each year, corresponding to the late growing season (pre-harvest period). This timing was chosen to capture the integrated effects of the mulching treatments after approximately six months of continuous interaction with the soil environment. Collected soil samples were homogenized, visible stones, plant residues, and roots were removed, and the samples were sealed and transported to the laboratory at low temperature for subsequent analysis. Samples from 2021 and 2022 were used for organic carbon analysis, and the 2022 samples were also used for metagenomic sequencing analysis.
2.3. Determination of Soil Carbon Fractions
Total organic carbon (TOC) was determined using a total organic carbon analyzer (TOC-L03030135, Shimadzu Corporation, Kyoto, Japan). Dissolved organic carbon (DOC) was determined using the water extraction method [28]. A total of 10 g of fresh soil was transferred to a 100 mL centrifuge tube, mixed with 50 mL of deionized water and shaken for 30 min, followed by centrifugation at 10,000 rpm for 10 min. The supernatant was filtered through a 0.45 μm glass fiber filter, and a blank control (without soil) was performed concurrently. Organic carbon in the filtrate was measured using total organic carbon analyzer.
Readily oxidizable carbon (ROC) was determined using the potassium permanganate oxidation method [29]. Air-dried soil (containing 15 mg C) sifted through a 500 μm sieve was placed in a 100 mL centrifuge tube, mixed with 25 mL of 333 mmol/L KMnO4, shaken at 200 rpm for 1 h, and centrifuged at 4000 rpm for 5 min. Then 0.4 mL of the filtrate was transferred to a 100 mL volumetric flask and diluted to volume. The absorbance at 565 nm was measured by a spectrophotometer (Cary 60 UV-Vis; Agilent Technologies, Santa Clara, CA, USA).
Particulate organic carbon (POC) was isolated following the method of Cambardella and Elliott [30] with minor modifications. Briefly, 10 g of air-dried soil (<2 mm) was dispersed in 30 mL of 5 g/L (NaPO3)6 solution in a 50 mL plastic bottle, and the mixture was shaken for 18 h. The dispersed soil slurry was then washed onto a set of nested sieves (250 μm and 53 μm) with tap water until the effluent was clear of fine particles. The material retained on the 53 μm sieve was transferred to pre-weighed aluminum boxes, dried at 60 °C and weighted. The organic carbon content of this fraction was subsequently determined by the potassium dichromate-sulfuric acid external heating method [31].
Light fraction organic carbon (LFOC) was determined using NaI separation according to Hamond et al. [32]. After sifting the fresh soil through a 2 mm sieve, 25 g of soil was weighed and placed in a 150 mL conical flask. A total of 50 mL of NaI solution with a density of 1.70 g/mL was added, and the mixture was shaken at 200 rpm/min for 1 h, then centrifuged at 2500 r/min for 20 min. The light fraction floating on the NaI surface was decanted onto a filter equipped with a 0.45 μm fiber membrane and vacuum filtered, then washed three times with 100 mL of 0.01 mol/L CaCl2 and 100 mL of distilled water. The extraction was repeated twice. The combined light fraction was dried at 60 °C, weighed, ground, and sifted through a 0.25 mm sieve. The organic carbon content was measured using the potassium dichromate-sulfuric acid external heating method.
Microbial biomass carbon (MBC) was determined using the chloroform fumigation method [33]. A total of 7.5 g of fresh soil sifted through a 2 mm sieve was placed in an aluminum box. A small beaker containing chloroform with glass beads, as well as a beaker containing water and dilute NaOH were placed in a vacuum desiccator. After evacuation, the chloroform was boiled vigorously for 3–5 min, then the desiccator valve was closed, and the sample was left in the dark for 24 h. After fumigation, chloroform was removed completely in a fume hood. Fumigated soil was transferred to a 150 mL flask, extracted with 30 mL of 0.5 mol/L K2SO4 (soil: water ratio = 1:4, w/w), shaken for 30 min, and filtered. Unfumigated soil was used as a blank control following the same procedure. The organic carbon content was measured using the potassium dichromate-sulfuric acid external heating method.
The contents of hardly oxidizable carbon (HOC), mineral-associated organic carbon (MOC) and heavy fraction organic carbon (HFOC) were calculated according to Equations (1)–(3):
2.4. Metagenomic Sequence and Analysis
Genomic DNA was extracted from soil samples using the HiPure Bacterial DNA Kit (Gene Denovo Biotechnology Co., Ltd, Guangzhou, China) according to the instructions. DNA quality was assessed using Qubit (Thermo Fisher Scientific, Waltham, MA, USA) and Nanodrop (Thermo Fisher Scientific, Waltham, MA, USA) [34].
Qualified genomic DNA was fragmented to approximately 350 bp by sonication, followed by end repair, A-tailing, and addition of Illumina sequencing adapters using the NEBNext® Ultra™ DNA Library Prep Kit (NEB, Ipswich, MA, USA). DNA fragments of 300–400 bp were enriched by PCR amplification. PCR products were purified using the AMPure XP system (Beckman Coulter, Brea, CA, USA). Sequencing libraries were evaluated using an Agilent 2100 Bioanalyzer (Agilent, Santa Clara, CA, USA), and library quantification was performed using real-time PCR. Sequencing was conducted on an Illumina Novaseq 6000 platform using a PE150 sequencing strategy [35].
Metagenomic data were filtered from raw reads generated on the Illumina platform using FASTP (version 0.18.0) [36]. Clean reads from each sample were assembled using MEGAHIT (version 1.1.2), and the resulting contiguous sequences were designated as contigs. Gene prediction was performed on contigs longer than 500 bp using MetaGeneMark (version 3.38). All gene sequences longer than 300 bp were selected, and CD-HIT (version 4.6) was used to cluster sequences with >95% similarity and >90% read coverage into clusters. Assembly metrics and mapping statistics for the sequencing data have been included in Supplementary Material Table S1 The longest sequence in each cluster was selected as the representative sequence (unigene) [37]. Reads were realigned to unigenes using Bowtie (version 2.2.5) and read counts were tallied. Genes with read support less than 2 were filtered out, and the resulting unigenes constituted the non-redundant gene set [38]. For gene abundance calculation, based on the alignment results obtained from Bowtie2 and with consideration of the number of mapped reads, gene length, and sequencing depth, the relative abundance of each Unigene in a given sample was computed according to Equation (4):
In the abundance calculation, Gi denotes the relative abundance of gene i in a given sample, Ri represents the number of reads mapped to gene i and Li is the length of gene i.
Unigenes were aligned and annotated against the Nr and KEGG databases (Kyoto Encyclopedia of Genes and Genomes, version 20200416) using Diamond (version 0.9.24), and carbohydrate-active enzyme annotation was performed based on the CAZy database (Carbohydrate-Active enZYmes Database, version 20210729). Taxonomic annotation at various levels was performed on clean reads using Kaiju (version 1.6.3) based on the Refseq database. Species annotation of genes was performed using MEGAN (version 6.19.9) based on the Lowest Common Ancestor (LCA) algorithm. The functional abundances for KEGG and CAZy categories were obtained by summing the relative abundances of the constituent Unigenes, with both annotation systems employing the same abundance calculation and normalization strategy [39,40].
2.5. Statistical Analysis
Soil carbon fraction data were organized in Microsoft Office Excel 2017, analyzed using IBM SPSS Statistics 21, and graphed using GraphPad Prism (version 6.01) and Origin 2021. Two-way ANOVA and Duncan’s multiple range test were applied on organic carbon fractions, with p < 0.05 considered statistically significant. Multiple comparison tests were performed only on samples within the same category. Microbial diversity analysis was conducted on the Omicsmart platform (http://www.omicsmart.com). For the differential analysis of functional pathways across groups, pairwise comparisons among the three groups (control vs. BLF, control vs. GBM, and BLF vs. GBM) were performed using Welch’s t-test. A p-value of less than 0.05 was considered statistically significant. The Benjamin–Hochberg (BH) method was used to calculate the q-values (FDR-corrected p-values) for each pair of comparison within each group. Redundancy analysis (RDA) was performed using Canoco 5, focusing on the top 10 abundant microbial phyla.
3. Results
3.1. Effect of Mulching on Organic Carbon Fractions
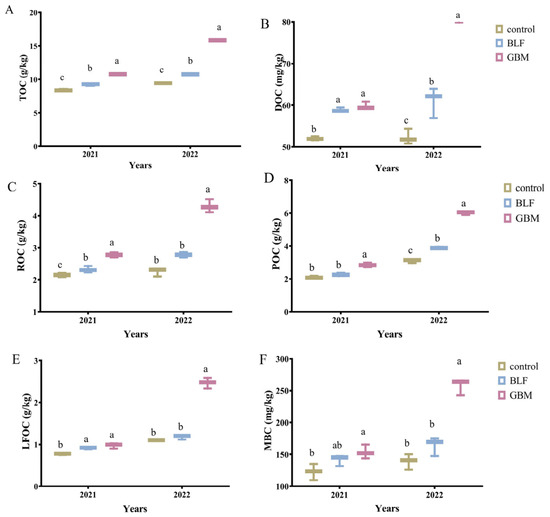
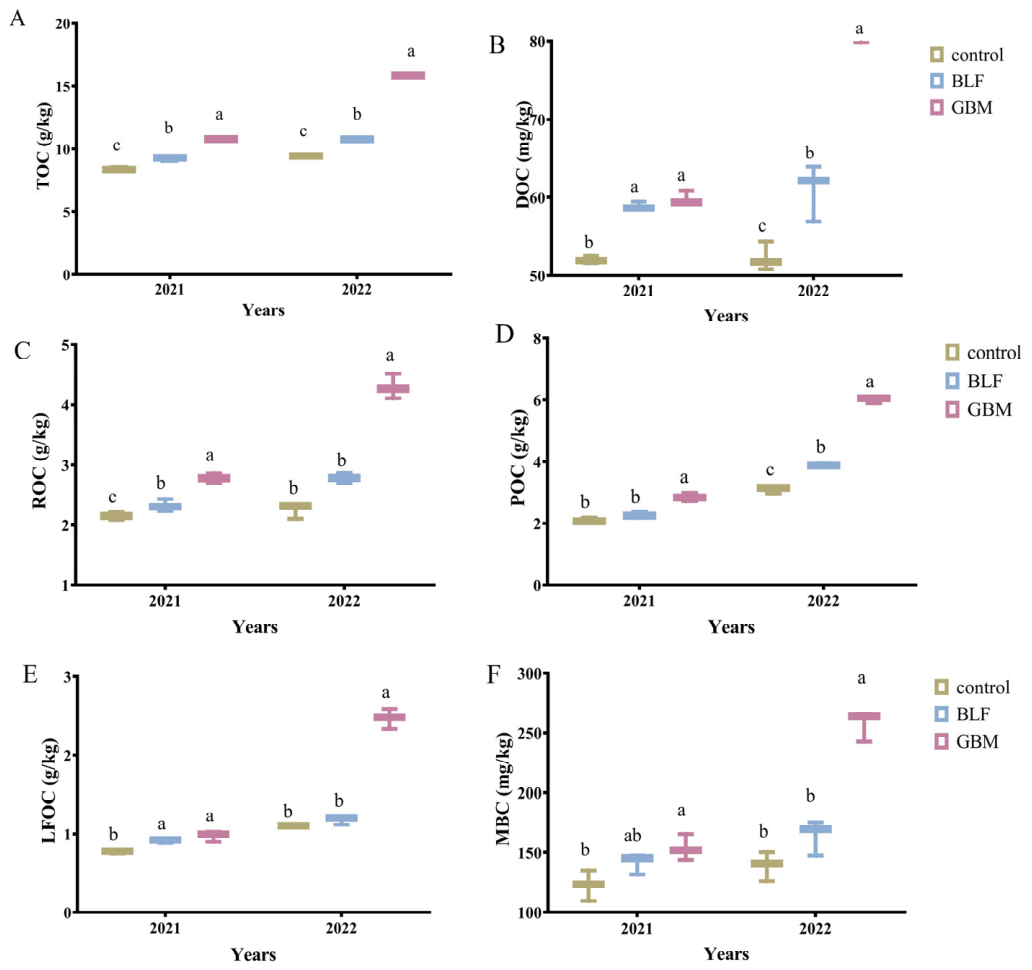
Changes in labile organic carbon fractions under different mulching treatments are shown in Figure 1. Compared with the control, BLF and GBM significantly increased total organic carbon (TOC) of soil in both years, with GBM consistently exceeding BLF (p < 0.05). The BLF treatment significantly increased soil DOC content, by 13.21% and 16.61% in 2021 and 2022, respectively, while it had a significant effect on the four active organic carbon fractions—ROC, POC, LFOC, and MBC—in only one of the two years. GBM treatment significantly increased the contents of all five labile organic carbon fractions. In the two years, the DOC contents in the GBM treatment were 15.09% and 56.72% higher than those in the control, respectively; ROC content increased by 10.76% and 90.27%, POC content by 35.71% and 93.87%, LFOC content by 25.97% and 124.55%, and MBC content by 25.20% and 85.11%, respectively.
Figure 1.
Labile organic carbon content under different treatments. (A) Total organic carbon (TOC); (B) dissolved organic carbon (DOC); (C) readily oxidizable carbon (ROC); (D) particulate organic carbon (POC); (E) light fraction organic carbon (LFOC); (F) microbial biomass carbon (MBC). Different lowercase letters indicate significant differences (p ≤ 0.05).
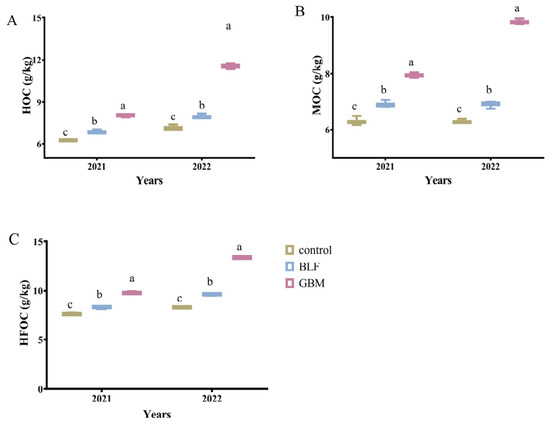
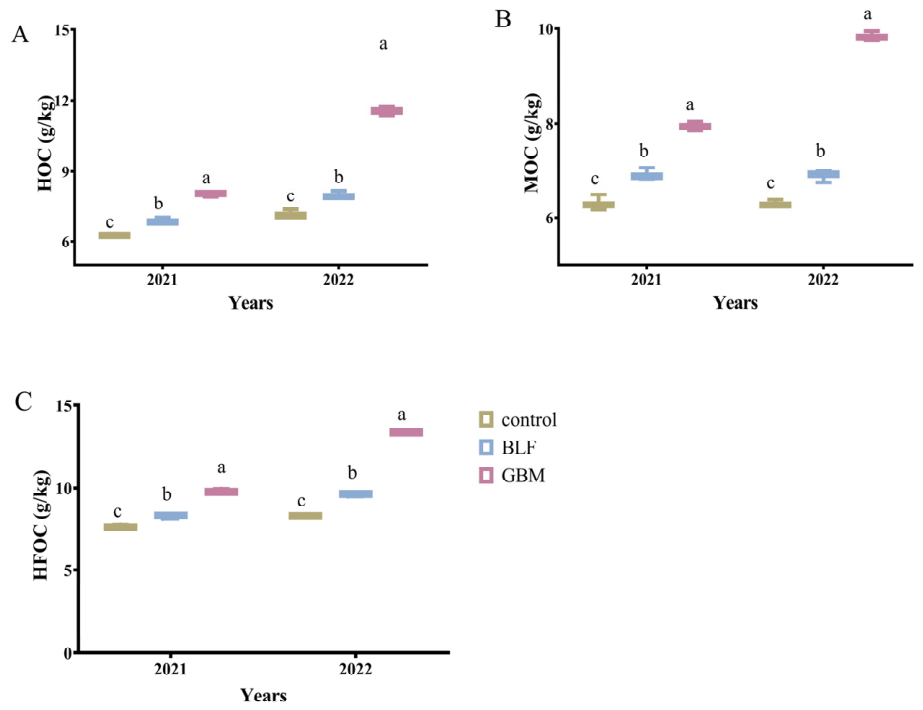
The changes in the content of recalcitrant organic carbon fractions under different mulching treatments are shown in Figure 2. Across both experimental years, mulching treatments significantly increased the three recalcitrant organic carbon content (p ≤ 0.05), with consistent trends among treatment groups: GBM > BLF > control. Compared to the control, the content of HOC in the GBM treatment increased by 28.12% and 61.40% in 2021 and 2022, respectively, while in the BLF treatment, it increased by 9.90% and 11.89%, respectively. The content of MOC increased by 25.83% and 55.92% in the GBM treatment and by 9.83% and 9.35% in the BLF treatment, respectively. The content of HFOC increased by 28.53% and 61.01% in the GBM treatment and by 8.38% and 15.64% in the BLF treatment, respectively. For the TOC and eight organic carbon fractions, both year and treatment had significant main effects (p < 0.05), with a significant interaction observed between the two factors (p < 0.05), indicating a second-order interaction effect on organic carbon content (Table 1).
Figure 2.
Recalcitrant organic carbon content under different treatments. (A) Hardly oxidizable carbon (HOC); (B) mineral-associated organic carbon (MOC); (C) heavy fraction organic carbon (HFOC). Different lowercase letters indicate significant differences (p ≤ 0.05).
Table 1.
Results of two-way ANOVA for content of labile organic carbon.
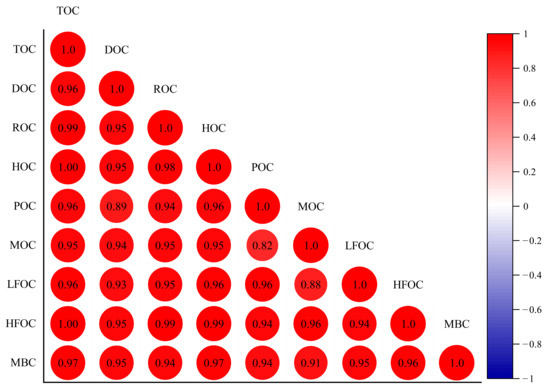
The proportions of five labile organic carbon fractions and three recalcitrant organic carbon fractions relative to total organic carbon were further analyzed (Table 2). Both mulching treatments increased the proportion of ROC, POC, and LFOC in soil organic carbon in 2022. GBM treatment had the greatest effect, increasing these proportions by 13.13%, 15.02%, and 32.76%, respectively. BLF treatment also significantly increased the proportion of LFOC in 2021. Both mulching treatments reduced the proportions of HOC and MOC in 2022. Compared to the control, GBM and BLF reduced the HOC proportion by 4.14% and 2.41%, and the MOC proportion by 7.38% and 4.56%, respectively. Correlation analysis between total soil organic carbon and individual organic carbon fractions (Figure 3) showed that each fraction was significantly positively correlated with total soil organic carbon, and inter-fraction correlations were also significantly positive, with Pearson’s correlation coefficients exceeding 0.9. Notably, soil organic carbon was highly correlated with the recalcitrant fractions HOC and HFOC.
Table 2.
Proportion of soil organic carbon fraction under different treatments.
Figure 3.
Pearson correlation analysis between organic carbon fractions.
3.2. Metagenomic Sequencing Analysis of Mulching Effects on Microbial Community Structure
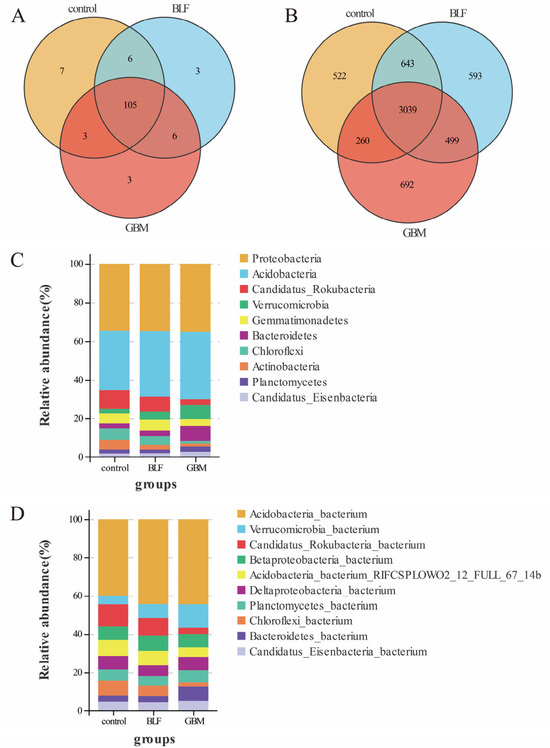
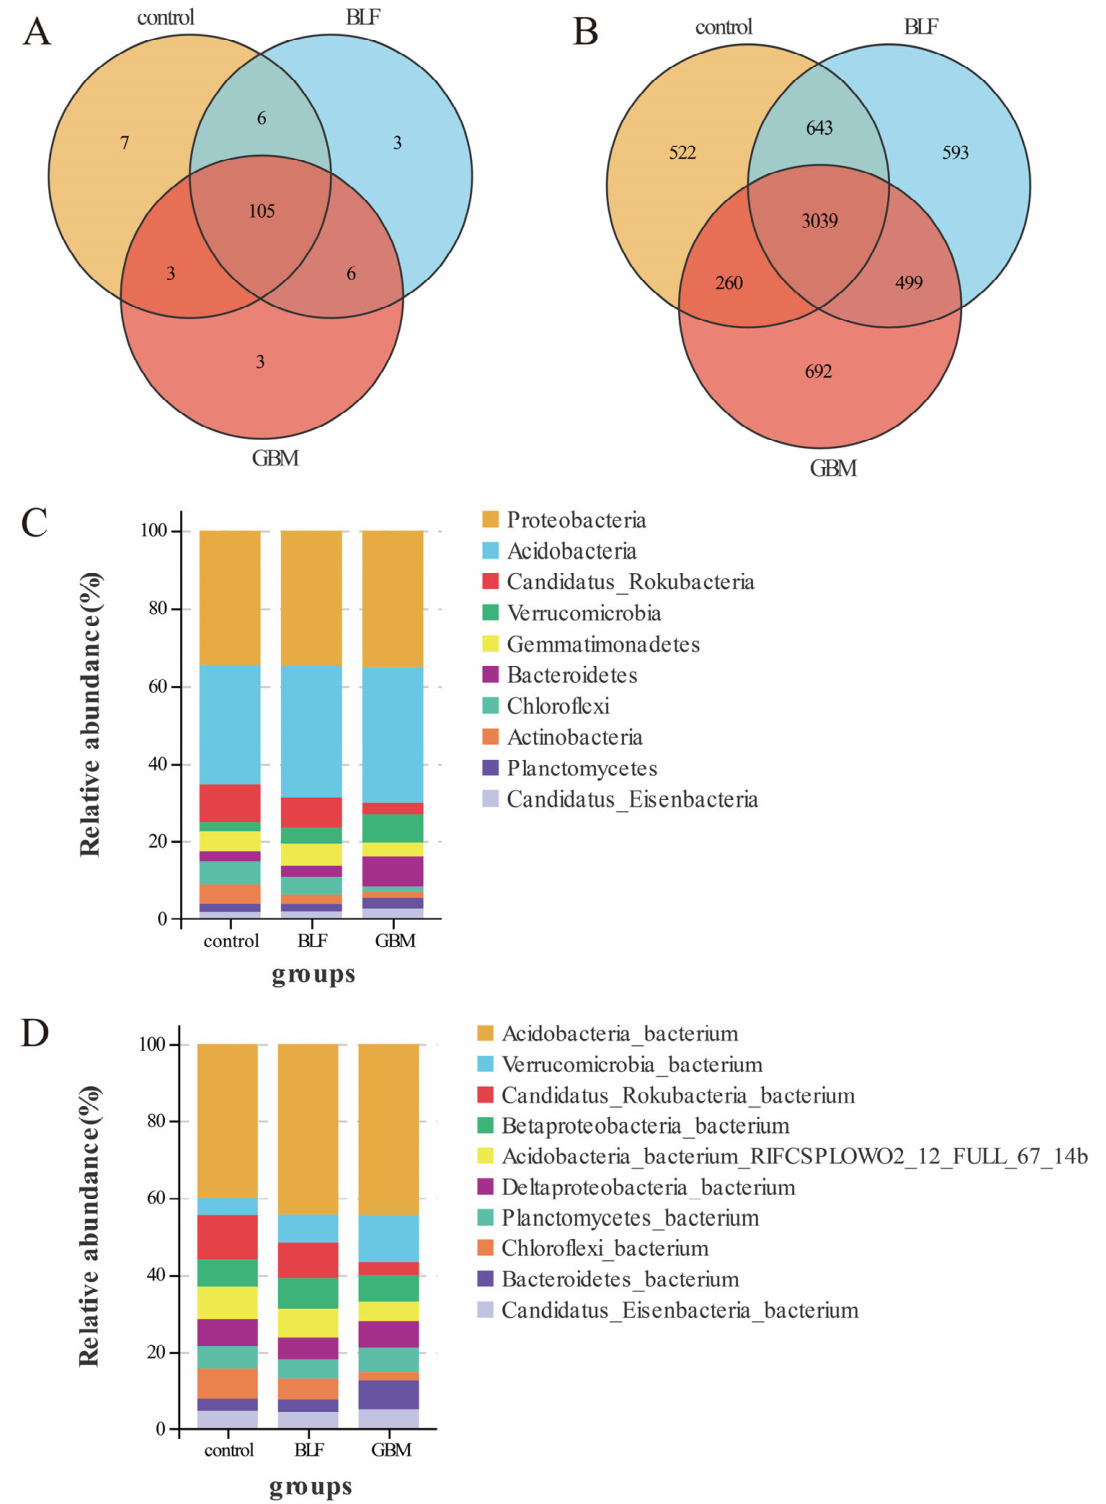
Soil microbial community structure and composition under different mulching treatments were analyzed based on metagenomic sequencing. A total of 133 microbial phyla were identified across the three soil groups (Figure 4A). Venn diagram analysis showed that the control, BLF, and GBM groups contained seven, three, and three unique microbial phyla, respectively, with 105 phyla shared among all three groups. Six microbial phyla were identified in GBM and BLF but not in the control, Abawacabacteria, Chisholmbacteria, Gracilibacteria, Portnoybacteria, Shapirobacteria, and Taylorbacteria, suggesting these may be key phyla influenced by mulching. A total of 4248 microbial species were identified across the three soil groups (Figure 4B). Among these, the control, BLF, and GBM groups contained 522, 593, and 692 unique species, respectively, with 3039 species shared among all groups.
Figure 4.
Analysis of the variations in soil microbial species in response to different mulching treatments. (A) The number of microbiological phyla; (B) the number of microbiological species; (C) distribution of the top 10 most abundant microorganisms at the phylum level; (D) top 10 abundant microorganisms at the soil microbial species level.
At the phylum level, the top 10 dominant bacterial phyla in terms of relative abundance were Proteobacteria, Acidobacteria, Candidatus Rokubacteria, Verrucomicrobia, Gemmatimonadetes, Bacteroidetes, Chloroflexi, Actinobacteria, Planctomycetes, and Candidatus Eisenbacteria under both mulching and clean tillage conditions (Figure 4C). However, relative abundances and orders of these phyla varied among treatments. Mulching showed an increasing trend of the abundance of Acidobacteria, Verrucomicrobia, Bacteroidetes, and Candidatus Eisenbacteria, while decreasing the abundance of Candidatus Rokubacteria, Chloroflexi, and Actinobacteria. Additionally, BLF tended to increase Gemmatimonadetes abundance and decrease Planctomycetes abundance, while GBM showed the opposite trend. At the species level, the top 10 dominant species were Acidobacteria bacterium, Verrucomicrobia bacterium, Candidatus Rokubacteria bacterium, Betaproteobacteria bacterium, Acidobacteria bacterium RIFCSPLOWO2_12_FULL_67_14b, Deltaproteobacteria bacterium, Planctomycetes bacterium, Chloroflexi bacterium, Bacteroidetes bacterium, and Candidatus Eisenbacteria bacterium (Figure 4D). Both mulching treatments increased the abundance of Acidobacteria bacterium, Verrucomicrobia bacterium, Betaproteobacteria bacterium, and Bacteroidetes bacterium, while decreasing the abundance of Candidatus Rokubacteria bacterium, Acidobacteria bacterium RIFCSPLOWO2_12_FULL_67_14b, and Chloroflexi bacterium. Moreover, the abundances of Deltaproteobacteria bacterium, Planctomycetes bacterium, and Candidatus Eisenbacteria bacterium decreased under BLF but increased under GBM.
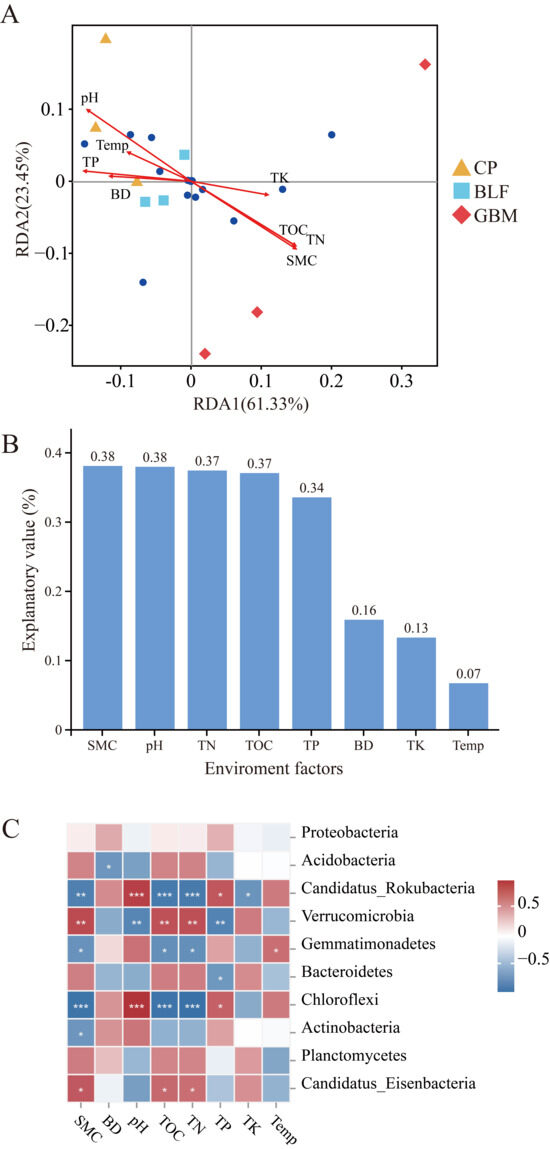
Redundancy analysis (RDA) was employed to investigate the potential relationships and potential regulatory mechanisms between environmental factors and microbial communities under two cover treatments and a control condition. The average pH values for the control, BLF, and GBM treatments in 2022 were 8.38, 8.29, and 8.16, respectively (Table S2). The other seven environmental factors were derived from the previous report by Duan [23], including soil temperature (Temp), soil moisture content (SMC), bulk density (BD), pH, total organic carbon (TOC), total nitrogen (TN), total phosphorus (TP), and total potassium (TK). The RDA was conducted at the phylum level.
The results showed that the cumulative contribution rate of the two axes was 84.78%, with the first axis contributing 61.33% and the second axis contributing 23.45% (Figure 5A). SMC, pH, TOC, TN, and TP were significantly correlated with differences in microbial community structure. SMC and pH showed the strongest correlations with microbial community structure, at 0.9039 and 0.9207, respectively. Furthermore, BD, pH, and TP had a greater influence on microbial community variation in the BLF samples. In contrast, the GBM sample points were scattered, and the RDA constraint axes provided poor explanatory power for them. To quantify the relative contribution of different environmental factors to the observed variation in microbial community composition, the Variable Partitioning Analysis (VPA) method was employed (Figure 5B). SMC, pH, TN, and TOC each contributed more than 35% to the total variation in microbial community composition. A Pearson correlation analysis was conducted between the top 10 most abundant microbial phyla and environmental factors (Figure 5C). The results showed that, with the exception of Proteobacteria and Planctomycetes, all other microbial groups were significantly correlated with environmental factors. In particular, Candidatus Rokubacteria, Verrucomicrobia, and Chloroflexi were significantly correlated with nearly all environmental factors. Among the eight environmental factors, SMC, TOC, and TN were the key factors influencing the abundance of dominant microbial groups.
Figure 5.
(A) Redundancy analysis between environmental factors and microbial communities under different mulching treatments. Blue dots denote the top 20 most abundant species at phylum level, while sample points in distinct colors represent different grouping information, arrows radiating from the origin indicate various environmental factors; (B) quantifying the relative contribution of environmental factors to changes in microbial community composition using the VPA method; (C) Pearson correlation analysis between the top 10 most abundant microbial phyla and environmental factors. ‘*’ means the two indicators are significantly different at the 0.05 level (p < 0.05); ‘**’ means p < 0.01; ‘***’ means p < 0.001.
3.3. KEGG Functional Analysis of Microbial Communities Under Mulching Conditions
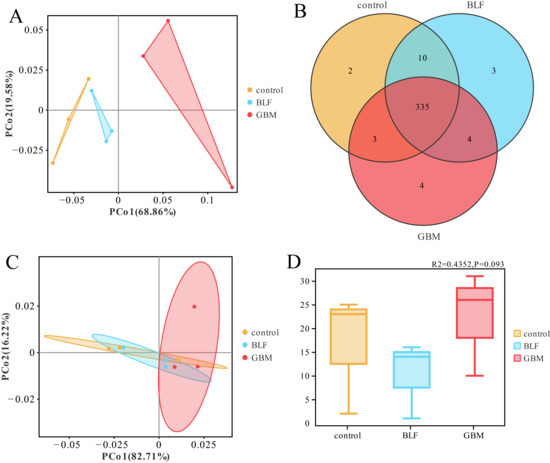
Principal coordinate analysis (PCoA) based on Bray–Curtis distances at different taxonomic levels was performed to examine differences in sample community composition (Figure 6A). The first two principal coordinates explained 88.44% of the total variation, indicating they adequately captured most information from the soil samples. The three groups of soil samples were clearly separated, indicating significant differences in microbial communities among treatments, with GBM showing greater divergence from the other two groups.
Figure 6.
Analysis of soil microbial β-diversity under different mulching treatments. (A) PCoA of soil microbial communities; (B) Venn analysis of the variations in soil microbial KEGG function; (C) PCoA of soil microbial metabolic pathways; (D) Adonis analysis of soil microbial metabolic pathways. Note: In (A,C), the shaded regions in different colors represent the confidence intervals for each group of samples. In (D), the boxes illustrate the magnitude of within‑group sample variation. The upper and lower bounds of each box correspond to the upper and lower quartiles, respectively, and the horizontal line inside the box marks the median.
KEGG enrichment analysis was performed on the genes detected in the soil samples to compare metabolic pathway differences among the three mulching treatments. A total of 361 metabolic pathways were enriched in the annotated dataset (Figure 6B). Among these, the control, BLF, and GBM groups contained 2, 3, and 4 unique metabolic pathways, respectively, with 335 pathways shared among all three groups. PCoA based on Bray–Curtis distances was performed to examine differences in metabolic pathways among samples (Figure 6C). The first two principal coordinates explained 98.93% of the total variation, indicating they adequately captured most information. However, the ellipses overlapped significantly, making it difficult to determine whether significant differences existed among the three groups. Further Adonis analysis of KEGG metabolic pathways, with permutation tests for statistical significance of grouping factors (Figure 6D), indicate a marginally significant effect, p = 0.093, with a variance contribution (R2) of 0.4352.
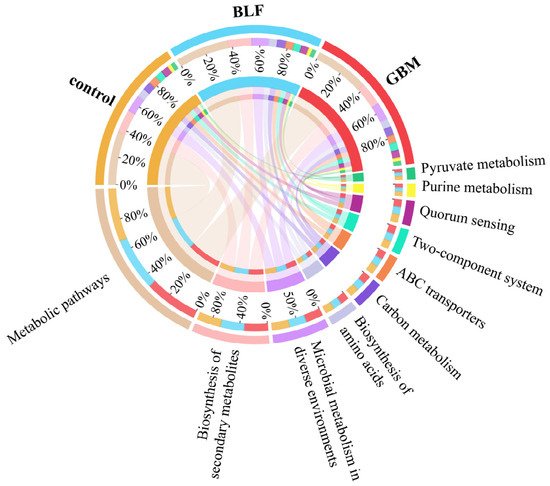
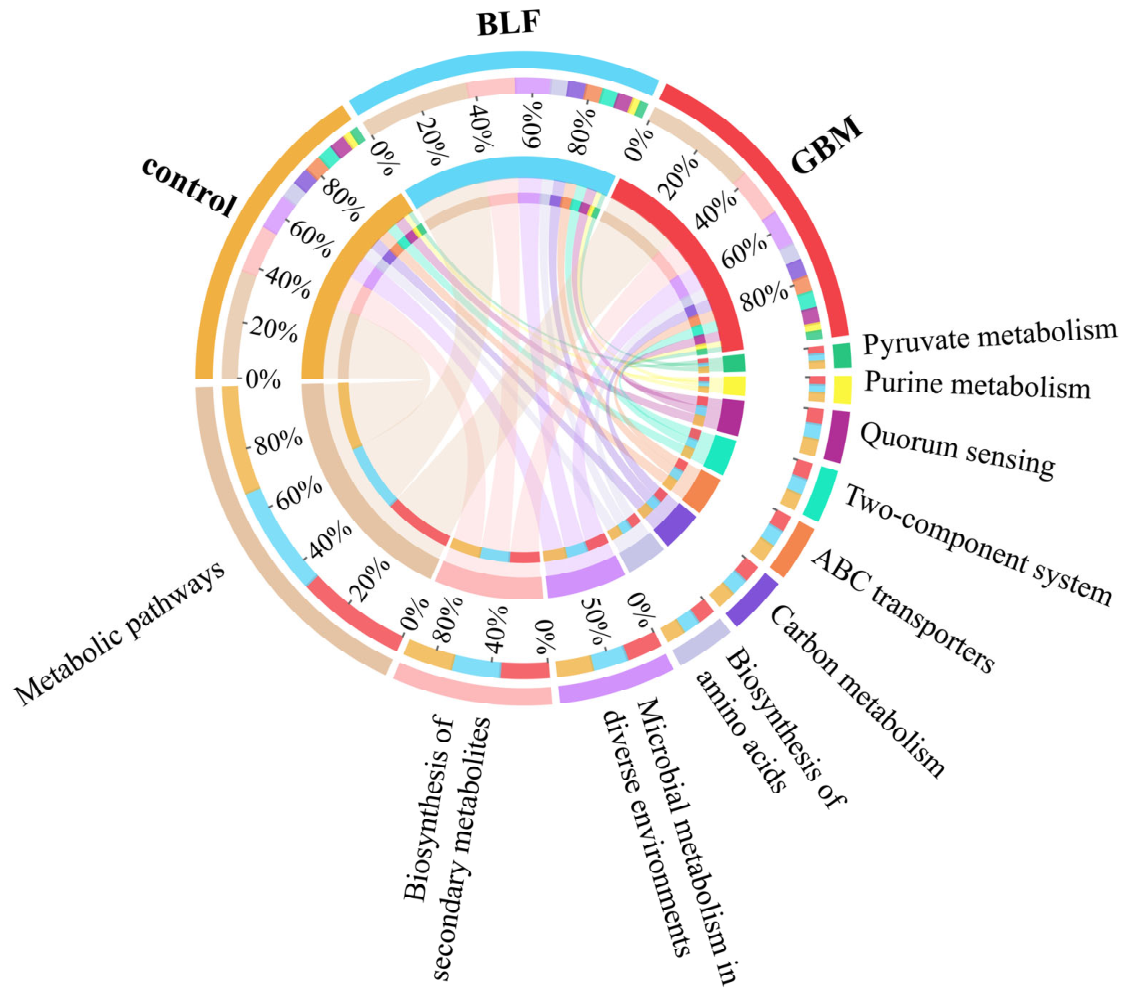
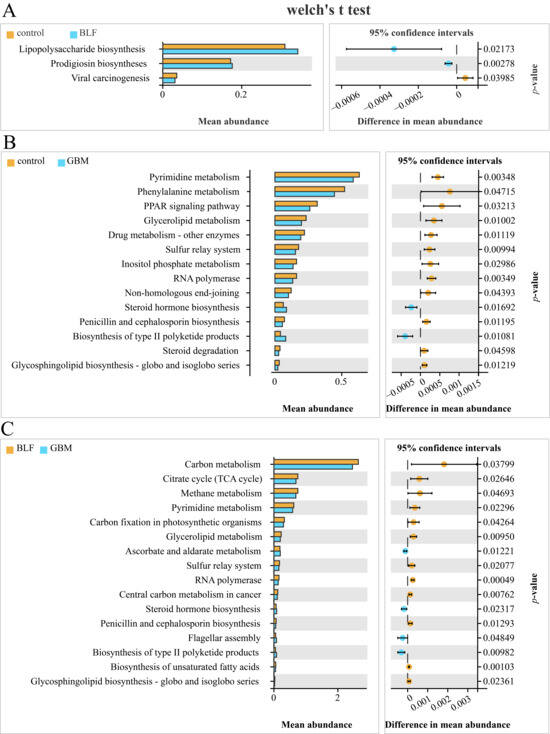
The top 10 metabolic pathways by abundance are shown in Figure 7, including metabolic pathways (ko01100), biosynthesis of secondary metabolites (ko01110), microbial metabolism in diverse environments (ko01120), biosynthesis of amino acids (ko01230), carbon metabolism (ko01200), ABC transporters (ko02010), two-component system (ko02020), quorum sensing (ko02024), purine metabolism (ko00230), and pyruvate metabolism (ko00620). No significant differences were observed in the top 10 metabolic pathways by abundance among the three treatment groups. After conducting pairwise comparisons among groups, Welch’s test identified the metabolic pathways that tend to be altered by the mulching treatments (Figure 8). In the three comparison groups—control vs. BLF, control vs. GBM, and BLF vs. GBM—3, 14, and 16 pathways with significant differences (p < 0.05) were identified, respectively, but no KEGG pathway met the significance threshold of q < 0.05 in any of the three pairwise comparisons. Several of these pathways are related to the carbon cycle, with carbon metabolism showing the highest abundance. The functions of genes related to carbon metabolism were further analyzed.
Figure 7.
Top 10 KEGG pathways by abundance in soil microbial communities under different mulching treatments.
Figure 8.
Metabolic pathways with significant differences in abundance under different mulching treatments. (A) Welch’s test between control and BLF; (B) Welch’s test between control and GBM; (C) Welch’s test between BLF and GBM.
3.4. Effects of Mulching on Functional Traits Related to Soil Microbial Carbon Cycling
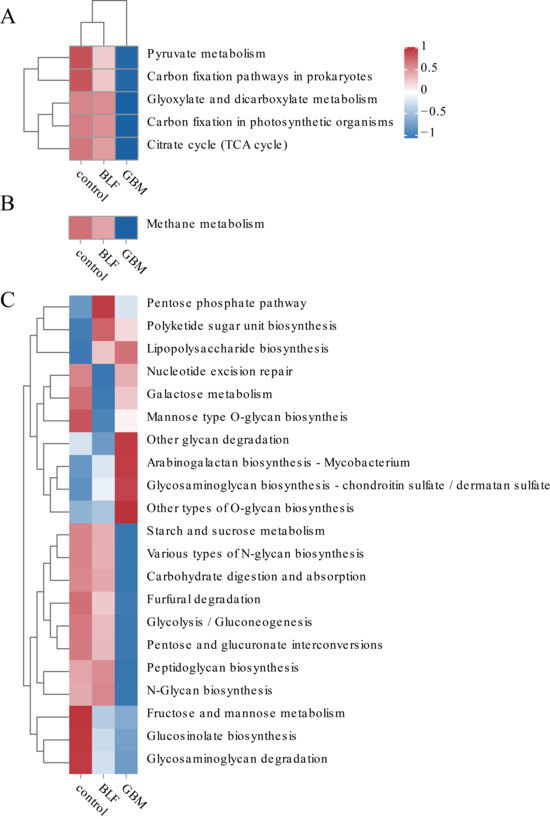
Microorganisms participate in multiple important carbon cycling processes, such as soil carbon fixation, methane metabolism, and carbohydrate metabolism. A cluster analysis was performed on carbon cycle-related metabolic pathways identified in this study (Figure 8). Mulching affected multiple metabolic pathways related to soil microbial carbon cycling. Five pathways associated with soil microbial carbon fixation, including pyruvate metabolism, carbon fixation pathways in prokaryotes, glyoxylate and dicarboxylate metabolism, carbon fixation in photosynthetic organisms, citrate cycle, and methane metabolism were decreased after mulching, with the trend being control > BLF > GBM (Figure 9A,B).
Figure 9.
Clustering heatmap of carbon cycle-related metabolic pathways under different mulching treatments. (A) Soil carbon fixation-related metabolic pathways; (B) soil methane metabolic pathways; (C) soil carbohydrate metabolism-related pathways.
KEGG analysis also identified twenty-one pathways related to carbohydrate metabolism (Figure 9C), and six of these were upregulated under both covering treatments, including pentose phosphate pathway, polyketide sugar unit biosynthesis, lipopolysaccharide biosynthesis, arabinogalactan biosynthesis–mycobacterium, glycosaminoglycan biosynthesis–chondroitin sulfate/dermatan sulfate, and other types of O-glycan biosynthesis. Several pathways related to carbohydrate metabolism were downregulated under both covering treatments, including starch and sucrose metabolism, various types of N-glycan biosynthesis, carbohydrate digestion and absorption, furfural degradation, glycolysis/gluconeogenesis, pentose and glucuronate interconversions, fructose and mannose metabolism, glucosinolate biosynthesis, and glycosaminoglycan degradation. The abundance of related genes in those pathways decreased after mulching, with the trend being control > BLF > GBM. Other pathways exhibit different responses under the two mulching treatments. In summary, GBM treatment significantly increased the abundance of functional genes related to glycan degradation, arabinogalactan biosynthesis, glycosaminoglycan biosynthesis, and O-glycan biosynthesis, and decreased the abundance of genes related to starch and sucrose metabolism, various types of N-glycan biosynthesis, carbohydrate digestion and absorption, furfural degradation, glycolysis/gluconeogenesis, pentose and glucuronate interconversions, peptidoglycan biosynthesis, N-glycan biosynthesis, fructose and mannose metabolism, glucosinolate biosynthesis, and glycosaminoglycan degradation. BLF treatment significantly increased the abundance of functional genes related to the pentose phosphate pathway and polyketide sugar unit biosynthesis, and decreased the abundance of genes related to nucleotide excision repair, galactose metabolism, and mannose type O-glycan biosynthesis.
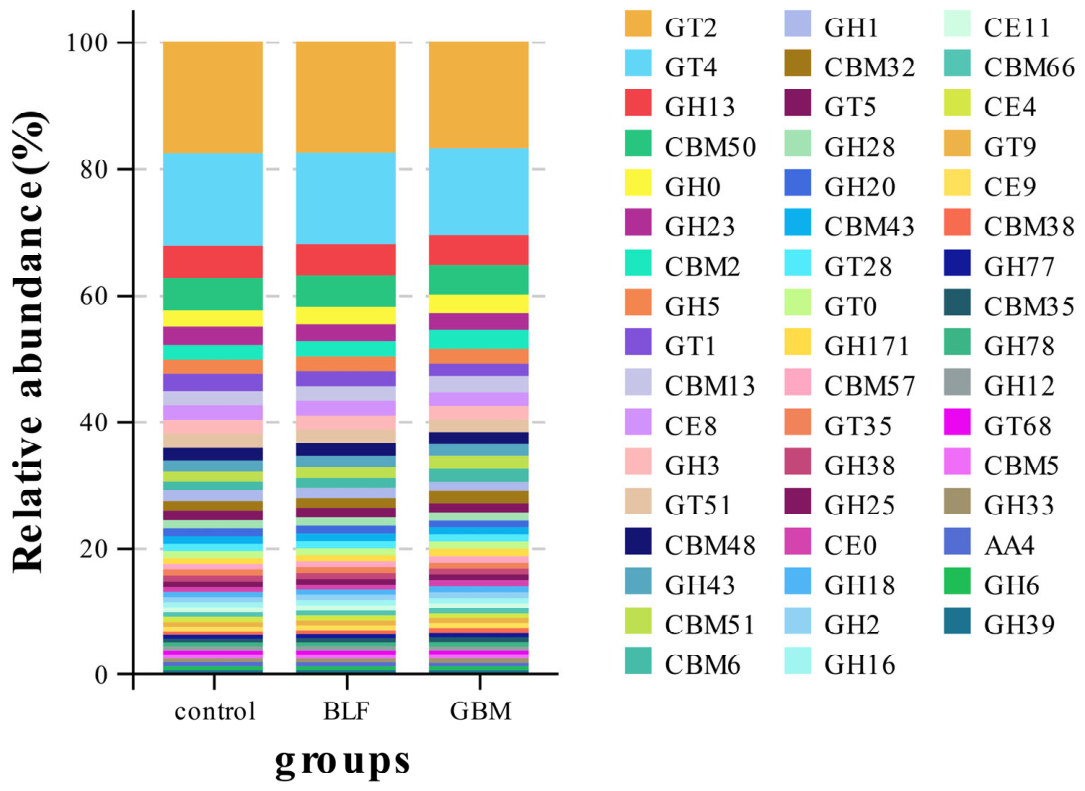
Analysis based on the CAZy database examined functional traits related to soil microbial carbon cycling under different mulching treatments. The CAZy database classifies carbohydrate-active enzymes into six functional modules: Glycosyl Transferases (GTs), Glycoside Hydrolases (GHs), Polysaccharide Lyases (PLs), Auxiliary Activities (AAs), Carbohydrate Esterases (CEs), and Carbohydrate-Binding Modules (CBMs). In this study, GT2 and GT4 were the dominant carbohydrate-active enzymes in all three soil groups. The top 50 most abundant CAZy gene families under different mulching treatments are shown in Figure 10, with greater differences observed between GBM and the control. The CAZy families most closely associated with lignocellulose degradation include GH1, GH3, GH5, GH9, GH48 (cellulases), GH10, GH11 (xylanases), and AA1, AA2, AA3 (auxiliary activity families involved in lignin modification). The results indicate that the abundances of these families did not differ significantly among the three treatments.
Figure 10.
Abundance of genes encoding carbohydrases under different mulching treatments.
Correlation analysis between soil carbon cycle-related metabolic pathways and soil organic carbon fractions (Figure 11) showed that all soil organic carbon fractions exhibited consistent correlations with carbon cycle-related pathways. Specifically, they were significantly positively correlated with O-glycan biosynthesis and significantly negatively correlated with pyruvate metabolism, N-glycan biosynthesis, carbon fixation in photosynthetic organisms, carbon fixation pathways in prokaryotes, the citrate cycle, furfural degradation, glyoxylate and dicarboxylate metabolism, methane metabolism, and peptidoglycan biosynthesis pathways.
Figure 11.
Pearson correlation analysis between soil carbon cycle-related pathways and organic carbon contents. Note: “*” means significant correlation (0.01 < p < 0.05), “**” means highly significant correlation (p < 0.01).
4. Discussion
4.1. Changes in Soil Organic Carbon Fractions Under Mulching Conditions
Soil organic carbon is divided into labile organic carbon (LOC) and recalcitrant organic carbon [41]. Labile organic carbon includes dissolved organic carbon (DOC), readily oxidizable carbon (ROC), particulate organic carbon (POC), light fraction organic carbon (LFOC), and microbial biomass carbon (MBC); recalcitrant organic carbon includes hardly oxidizable carbon (HOC), mineral-associated organic carbon (MOC), and heavy fraction organic carbon (HFOC). DOC reflects the potential for soil organic matter decomposition and is an important indicator of soil quality and function [42]. ROC has a relatively short turnover time, is closely related to soil nutrient supply and crop growth, serves as a major source of plant nutrients, and is considered an active indicator of soil organic matter [43]. Therefore, soil labile organic carbon can serve as an early indicator of changes in soil organic carbon and soil quality [44]. POC and LFOC originate primarily from plant residues and roots, with carbohydrates and amino acids as their main chemical components. Their levels increase with the addition of organic materials [45,46], reflecting the short-term effects of land use practices on organic carbon [47]. The biomass carbon of plant residues is a primary factor influencing MBC, as biomass carbon is a major carbon source for microorganisms [48,49]. Studies have shown that crop residues, as carbon source inputs, provide a substrate for soil microorganisms, enhance microbial activity, and thereby increase the labile components of the soil carbon pool [50]. Recalcitrant organic carbon components typically exist as bound complexes, are less accessible to microorganisms, represent stable carbon fractions in soil, and are mechanisms for soil organic carbon sequestration [51,52]. Exogenous organic carbon inputs primarily affect labile organic carbon fractions first, whereas changes in recalcitrant organic carbon content, due to its large molecular size and complex structure, require time for transformation and accumulation [53].
Organic mulch in orchards contributes to increase soil organic carbon (SOC) sequestration, primarily by increasing organic carbon inputs and reducing CO2 emissions [15,54]. Marks et al. (2022) reported that five years of inter-row mulching in vineyards increased SOC stocks by 22.7% and identified differences in the effects of various mulch materials on SOC and DOC [22]. This study used two organic materials commonly employed in production for in-row mulching in vineyards to evaluate their potential impact on soil carbon sequestration. Although GBM has a lower carbon content (45% of dry matter) than BLF (78% of dry matter), its application rate (10,000 kg fresh weight·ha−1) is substantially higher than that of BLF (300 kg liquid·ha−1). Consequently, the total carbon input from GBM (2790 kg C·ha−1) is approximately 17 times that of BLF (161 kg C·ha−1). This disparity arises from the different design philosophies of the two mulching strategies. GBM is a thick layer of organic mulch applied at high rates, whose primary function is to directly introduce large amounts of organic carbon into the soil and improve its physicochemical properties [25], whereas BLF is a thin film of functional mulch applied at low rates, primarily serving to regulate the water and heat balance and the microenvironment at the soil surface [23,55]. In addition, carbon in GBM primarily exists in the form of lignocellulosic structural carbon (cellulose, hemicellulose, and lignin). The high carbon-to-nitrogen ratio (51:1) results in slow decomposition of these substances, which contribute to both labile and recalcitrant soil organic carbon pools [15,56,57]. The results of this study also support this effect, as GBM treatment was shown to significantly increase both labile organic carbon (Figure 1) and recalcitrant organic carbon (Figure 2). In contrast, BLF had a significant effect only on the recalcitrant organic carbon fraction, while its effect on the labile organic carbon was dependent on the vintage, which may be related to the material properties. The carbon in BLF primarily originates from mineral raw materials and humic acid, with a portion existing in soluble form that is prone to leaching after application. Within the six months between treatment and sampling, the BLF material had already undergone natural degradation [58], and changes in recalcitrant organic carbon may be due to its persistent effects on soil properties and microbial communities [23,55].
The proportion of each organic carbon fraction relative to total organic carbon reveals the composition of the soil organic carbon pool and reflects its turnover [59]. In this study, both mulching treatments increased the proportions of labile fractions ROC, POC, and LFOC while decreasing the proportions of recalcitrant fractions HOC and MOC (Table 1). This indicates that, compared to the control, BLF and GBM treatments shifted the soil carbon pool toward a more active state, thereby accelerating organic carbon turnover. Significant changes in soil bulk density were observed under both mulching treatments, as previously reported in our earlier study [54]. Following the method described by Marks et al. (2022), soil carbon sequestration per unit area was calculated as the product of total organic carbon (TOC) content, soil bulk density, and sampling depth (20 cm) [22]. The results showed that GBM significantly increased soil SOC sequestration in both 2021 and 2022, whereas BLF exhibited a significant effect only in 2021 (Table S3). In summary, both BLF and GBM have been shown to have a positive impact on carbon sequestration, but there is a significant disparity between the two in terms of input and long-term effects. Therefore, it is crucial to investigate the soil characteristics of the production area and adjust the application rates and types of organic amendments based on the specific needs of vineyards. Whether appropriately increasing the application rate or frequency of BLF, or adjusting the carbon-to-nitrogen ratio of GBM, would enhance the decomposition and sequestration of carbon inputs is a question worthy of further research.
4.2. Analysis of Soil Microbial Community Structure Under Mulching Conditions
Metagenomic analysis revealed that the top 10 dominant phyla in relative abundance across the three soil groups were Proteobacteria, Acidobacteria, Candidatus Rokubacteria, Verrucomicrobia, Gemmatimonadetes, Bacteroidetes, Chloroflexi, Actinobacteria, Planctomycetes, and Candidatus Eisenbacteria (Figure 4). The relative abundances of these dominant phyla varied with mulching material. Proteobacteria and Acidobacteria consistently exhibited a relatively high trend among bacteria under both clean tillage and mulching, together accounting for over 70% of total abundance, indicating that the different mulching materials had little effect on the composition of dominant phyla but rather altered their abundances. The relative abundance of Planctomycetota in BLF and GBM was higher than in the control. Planctomycetes are oligotrophic bacteria capable of utilizing recalcitrant carbon sources and are also dominant nitrogen-fixing bacteria in soil [60,61,62]. They can secrete β-glucosidase and xylanase to participate in the decomposition of plant residues [63].
The differential effects of BLF and GBM on soil microbial communities and organic carbon fractions observed in this study may be attributed to two interconnected mechanisms: changes in the soil physical properties and the chemical composition of the materials. Mulching materials applied to soil surfaces universally modify the soil physical environment through multiple pathways. Both biodegradable film mulches and organic residue mulches have been shown to reduce soil bulk density and increase soil porosity, while simultaneously increasing soil moisture content through reduced evaporation and moderating soil temperature fluctuations via physical insulation [64,65,66,67]. These changes in soil physical properties create a more favorable microhabitat for soil microorganisms. Improved soil aeration, water availability, and thermal conditions enhance microbial activity and diversity [26,28]. The physical barrier effect of mulches also reduces surface evaporation and soil erosion, contributing to the preservation of soil organic carbon. RDA of environmental factors and microbial communities also showed that SMC, pH, TOC, TN, and TP were all significantly correlated with differences in microbial community structure (Figure 5).
In addition, the difference in the carbon-to-nitrogen ratio between the two materials may also be one of the factors influencing microbial communities and carbon distribution. The carbon-to-nitrogen ratio of the substrate is a key determinant of microbial degradation efficiency [68,69]. When microorganisms decompose substrates with a C:N ratio exceeding the microbial threshold elemental ratio (TER)—approximately 20:1—they assimilate mineral nitrogen from the soil to meet their stoichiometric requirements, a process known as nitrogen immobilization [68,69,70]. With a C:N ratio of 51:1, GBM substantially exceeds this threshold, inducing significant nitrogen immobilization during early decomposition stages. This nitrogen limitation reduces microbial carbon mineralization rates and slows overall decomposition [71]. Consequently, the large carbon input from GBM (2790 kg C·ha−1) is released gradually, contributing more to the accumulation of recalcitrant organic carbon fractions (HOC, MOC, and HFOC) observed in this study. Conversely, substrates with a low C:N ratio (such as BLF) can improve microbial carbon use efficiency (CUE) and promote faster carbon turnover [67,70]. Furthermore, substrate C:N ratio influences microbial community composition. During the decomposition of high C:N substrates, bacterial communities undergo succession—early stages are dominated by copiotrophic taxa (such as Bacilli and Proteobacteria), while later stages are dominated by oligotrophic taxa, including Acidobacteria [72]. Specific members of Acidobacteria (e.g., Bryocella and Candidatus Solibacter) have been identified as K-strategists adapted to resource-limited conditions and capable of decomposing complex organic compounds [73]. This mechanistic link explains the increased Acidobacteria abundance observed in GBM-treated soils in our metagenomic analysis, as well as the distinct carbon fraction distribution patterns.
4.3. Changes in Functional Traits Related to Soil Carbon Cycling Under Mulching Conditions
Soil carbon cycling, the process of transformation and migration of carbon among different forms in the soil, is one of the most important and complex biogeochemical cycles in soil ecosystems, playing a crucial role in maintaining soil fertility, protecting the environment, and regulating climate [74]. As key drivers of organic carbon cycling and fixation, the ecological functions of soil microorganisms have received increasing attention [13]. Soil carbon cycling is influenced by factors such as microbial physiology, organic compound types, and redox forms [75,76]. Because these interactions are highly complex, studying carbon cycling within microbial communities is challenging [77,78]. Microbial biomass is an important parameter in carbon degradation models, but it has limitations in explaining carbon decomposition processes by itself [79]. Studies have found that soil microbial community composition and structural characteristics can regulate the dynamics of the soil carbon pool and predict its long-term evolution [80,81].
This study employed whole-genome sequencing to analyze the soil microbiome under different mulching regimes and systematically annotated carbon cycle-related metabolic pathways based on the KEGG database, with a focus on functional gene abundances and their encoded enzyme systems related to carbon fixation, methane metabolism, and carbohydrate metabolism pathways (Figure 8). In soil carbon fixation and methane metabolism pathways, mulching reduced the abundance of related functional genes. However, among carbohydrate metabolism-related pathways, there were marked differences in the abundance of metabolic functional genes between the two mulched soils. Different mulching treatments altered the corresponding soil microbial compositions, thereby affecting the relative abundance of genes. This is because most functional processes in soil are regulated by microorganisms, and changes in microbial community function are closely linked to microbial community composition [82]. Notably, although the cover treatment upregulated certain carbohydrate synthesis-related pathways, such as the pentose phosphate pathway, lipopolysaccharide biosynthesis, and O-glycan biosynthesis, the majority of carbohydrate metabolic pathways—including glycolysis/gluconeogenesis, starch and sucrose metabolism, and various N-glycan biosynthesis pathways—exhibited a downregulated trend. This suggests that the impact of mulching on soil microbial carbon metabolism is not a straightforward “promotion” but rather a potential shift in microbial carbon substrate preferences and metabolic flux, redirecting from the decomposition and utilization of plant-derived polysaccharides toward the synthesis of microbial structural components [83]. Due to limitations in field trial conditions, the number of biological replicates for each treatment in this study was relatively limited. Therefore, differences in functional pathways among groups (Welch’s t-test, p < 0.05) should be considered preliminary findings, and their reliability requires further validation through studies with larger sample sizes.
Carbohydrate-active enzymes are a diverse group of enzymes involved in the synthesis and hydrolysis of carbohydrates, participating in nearly all metabolic processes of carbohydrates. Soil carbohydrate-active enzymes originate mainly from microorganisms, including fructosyltransferases, pectinases, and glucosyltransferases [84]. In this study, glycosyltransferases were the most abundant across all three soil groups. Soil carbon cycling functions result from the combined action of multiple microbial taxa. For example, Proteobacteria, Acidobacteria, and Actinobacteria are all major taxa involved in soil carbon reactions. Studies have also shown that they are major participants in nitrogen and phosphorus cycles [85,86]. Correlation analysis indicated that functional genes/metabolic pathways related to soil carbon cycling were significantly correlated with environmental factors (Figure 10), consistent with previous studies [87]. Furthermore, this study is based on the abundance of functional genes in the metagenome, reflect the potential for function, rather than actual enzyme activity or degradation rates. A systematic and quantitative assessment of lignocellulose degradation potential—linking the specific chemical composition of GBM (i.e., its high C:N ratio and lignin content) to the functional potential of the microbial community—is essential for a comprehensive interpretation of carbon cycling under GBM mulching. It should be noted that, in order to fully elucidate the functional activity of these pathways, future studies will need to combine transcriptomic or proteomic approaches with controlled degradation experiments.
5. Conclusions
This study demonstrates that two contrasting mulching strategies—GBM (high C input, high C:N) and BLF (low C input, low C:N)—differentially regulate soil organic carbon fractions, microbial communities, and carbon-cycle functional genes in a vineyard system. Both BLF and GBM treatments significantly increased recalcitrant organic carbon content, while GBM treatment also increased labile organic carbon content. The two mulching treatments increased the proportions of labile fractions ROC, POC, and LFOC and decreased the proportions of recalcitrant fractions HOC and MOC. Metagenomic sequencing analysis of soil microorganisms identified 133 phyla and 6248 species, with the highest relative abundances observed in the Proteobacteria, Acidobacteria, Actinobacteria, etc. The two mulching treatments significantly influenced the abundances of Acidobacteria, Verrucomicrobia, and Bacteroidetes. Metagenomic analysis confirmed that mulching downregulated carbon fixation and methane metabolism while upregulating carbohydrate metabolism pathways, with GBM exerting stronger effects on carbon-cycle enzyme genes. These two-year results represent preliminary observations on the SOC mutations that often occur very slowly in medium-to-long-term periods, providing a theoretical basis for understanding the relationship between soil microbial communities and the carbon cycle. Future studies that incorporate long-term, multi-temporal sampling will further elucidate the temporal patterns of carbon accumulation in vineyard systems and the response of microbial communities to cover measures.
Supplementary Materials
The following supporting information can be downloaded at https://www.mdpi.com/article/10.3390/horticulturae12070901/s1. Table S1: Assembly Metrics and Alignment Statistics for Metagenomic Sequencing Data; Table S2: The soil pH values for three treatments; Table S3: The SOC stocks for three treatments.
Author Contributions
Conceptualization, X.D. and L.Y.; methodology and resources, X.D. and X.H.; investigation, data curation, and software, X.H. and Y.L.; formal analysis and project administration, Y.W.; writing—original draft preparation, X.H.; writing—review and editing, X.D.; funding acquisition, L.Y. All authors have read and agreed to the published version of the manuscript.
Funding
This research was funded by Agricultural Science & Technology Innovation Project of Shandong Academy of Agricultural Sciences (CXGC2026B13).
Data Availability Statement
Raw sequence data of this article were deposited at BioSample database under accession number PRJNA1493102 (https://www.ncbi.nlm.nih.gov/sra/PRJNA1493102, accessed on 10 July 2026). Further inquiries can be directed to the corresponding authors.
Conflicts of Interest
The authors declare no conflicts of interest.
Appendix A
Figure A1.
Schematic diagram of vineyards with different mulching treatments. (A) Clean-tilled (control); (B) biodegradable liquid film mulch (BLF); (C) shredded grape branches mulch (GBM).
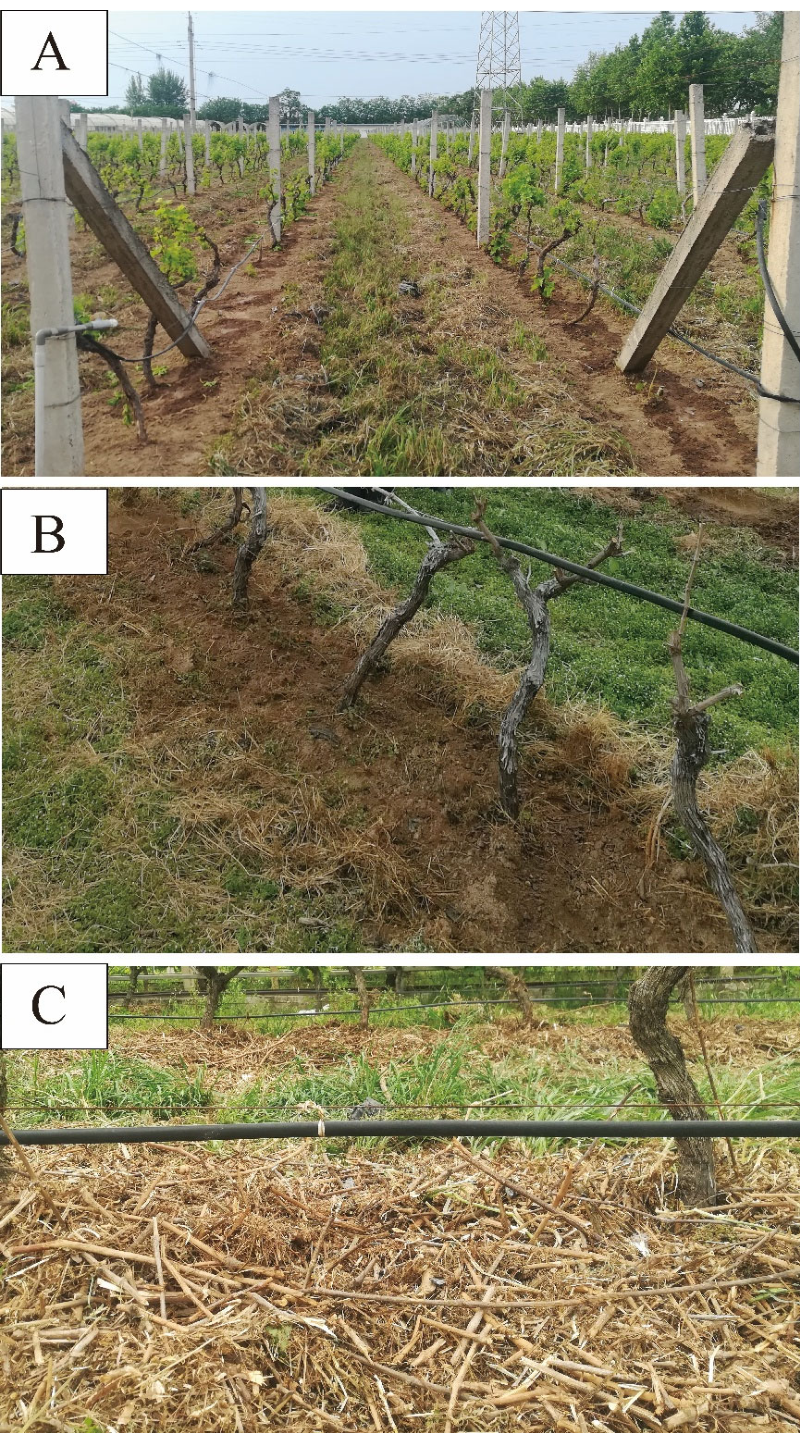
Figure A2.
The experimental setup of each block as replicate. Notes: Two rows per treatment. A total of 90 vines per row. The treatments were arranged in nonadjacent rows. The experimental setup had three such blocks.
References
- Vendrame, N.; Tezza, L.; Pitacco, A. Study of the carbon budget of a temperate-climate vineyard: Inter-annual variability of CO2 flux. Am. J. Enol. Vitic. 2019, 70, 34–41. [Google Scholar] [CrossRef] [Scilit]
- Liang, C.; Schimel, J.P.; Jastrow, J.D. The importance of anabolism in microbial control over soil carbon storage. Nat. Microbiol. 2017, 2, 17105. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Goward, J.W.M. Estimating and Predicting Carbon Sequestered in a Vineyard with Soil Surveys, Spatial Data and GIS Management. Master Thesis, University of New South Wales, Sydney, Australia, 2012; pp. 52–57. [Google Scholar]
- Jansson, J.K.; Hofmockel, K.S. Soil microbiomes and climate change. Nat. Rev. Microbiol. 2020, 18, 35–46. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Witzgall, K.; Vidal, A.; Schubert, D.I.; Höschen, C.; Schweizer, S.A.; Buegger, F.; Pouteau, V.; Chenu, C.; Mueller, C.W. Particulate organic matter as a functional soil component for persistent soil organic carbon. Nat. Commun. 2021, 12, 4115. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kallenbach, C.M.; Frey, S.D.; Grandy, A.S. Direct evidence for microbial-derived soil organic matter formation and its ecophysiological controls. Nat. Commun. 2016, 7, 13630. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liang, C.; Amelung, W.; Lehmann, J.; Kästner, M. Quantitative assessment of microbial necromass contribution to soil organic matter. Glob. Change Biol. 2019, 25, 3578–3590. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bardgett, R.D.; Van Der Putten, W.H. Belowground biodiversity and ecosystem functioning. Nature 2014, 515, 505–511. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dong, X.; Hao, Q.; Li, G.; Lin, Q.; Zhao, X. Contrast effect of long-term fertilization on SOC and SIC stocks and distribution in different soil particle-size fractions. J. Soils Sediments 2017, 17, 1054–1063. [Google Scholar] [CrossRef] [Scilit]
- Liu, Z.; Sun, Y.; Zhang, Y.; Feng, W.; Lai, Z.; Fa, K.; Qin, S. Metagenomic and 13C tracing evidence for autotrophic atmospheric carbon absorption in a semiarid desert. Soil Biol. Biochem. 2018, 125, 156–166. [Google Scholar] [CrossRef] [Scilit]
- Liu, Z.; Sun, Y.; Zhang, Y.; Feng, W.; Lai, Z.; Qin, S. Soil microbes transform inorganic carbon into organic carbon by dark fixation pathways in desert soil. J. Geophys. Res. Biogeosci. 2021, 126, e2020JG006047. [Google Scholar] [CrossRef] [Scilit]
- Don, A.; Böhme, I.H.; Dohrmann, A.B.; Poeplau, C.; Tebbe, C.C. Microbial community composition affects soil organic carbon turnover in mineral soils. Biol. Fertil. Soils 2017, 53, 445–456. [Google Scholar] [CrossRef] [Scilit]
- Liang, C.; Balser, T.C. Warming and nitrogen deposition lessen microbial residue contribution to soil carbon pool. Nat. Commun. 2012, 3, 1222. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- McBride, S.G.; Osburn, E.D.; Lucas, J.M.; Simpson, J.S.; Brown, T.; Barrett, J.E.; Strickland, M.S. Volatile and dissolved organic carbon sources have distinct effects on microbial activity, nitrogen content, and bacterial communities in soil. Microb. Ecol. 2023, 85, 659–668. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Rodrigo, E.; Mairata, A.; Martínez-Vidaurre, J.M.; Pou, A. Evaluating the role of organic mulches in reducing soil CO2 emissions and improving soil conditions in a commercial vineyard. Sci. Total Environ. 2025, 1000, 180441. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Baiamonte, G.; Minacapilli, M.; Novara, A.; Gristina, L. Time scale effects and interactions of rainfall erosivity and cover management factors on vineyard soil loss erosion in the semi-arid area of southern sicily. Water 2019, 11, 978. [Google Scholar] [CrossRef] [Scilit]
- Garcia, L.; Celette, F.; Gary, C.; Ripoche, A.; Valdés-Gómez, H.; Metay, A. Management of service crops for the provision of ecosystem services in vineyards: A review. Agric. Ecosyst. Environ. 2018, 251, 158–170. [Google Scholar] [CrossRef] [Scilit]
- Liu, Y.; Teng, Y.; Zheng, J.; Khan, A.; Li, X.; Cui, J.; Verma, K.K.; Guo, Q.; Zhu, K. The impact of long-term mulching cultivation on soil quality, microbial community structure, and fruit quality in “Wanzhou Red Mandarin” citrus orchard. Front. Microbiol. 2025, 16, 1616151. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Capó-Bauçà, S.; Marqués, A.; Llopis-Vidal, N.; Bota, J.; Baraza, E. Long-term establishment of natural green cover provides agroecosystem services by improving soil quality in a Mediterranean vineyard. Ecol. Eng. 2019, 127, 285–291. [Google Scholar] [CrossRef] [Scilit]
- Rocha, F.I.; Rodriguez-Ramos, J.C.; Fernando, M.; Hale, L. Interrow cover crops in a semi-arid vineyard increase plant beneficial functional potential of the soil microbiome, both in vine rows and interrows, a benefit that increases with cover crop duration. Environ. Microbiome 2025, 20, 66. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zumkeller, M.; Yu, R.; Torres, N.; Marigliano, L.E.; Zaccaria, D.; Kurtural, S.K. Site characteristics determine the effectiveness of tillage and cover crops on the net ecosystem carbon balance in California vineyard agroecosystems. Front. Plant Sci. 2022, 13, 1024606. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Marks, J.N.J.; Lines, T.E.P.; Penfold, C.; Cavagnaro, T.R. Cover crops and carbon stocks: How under-vine management influences SOC inputs and turnover in two vineyards. Sci. Total Environ. 2022, 831, 154800. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Duan, X.; Luo, T.; Ding, Y.; Han, X.; Li, H.; Wang, H. The impact of vineyard mulch on soil quality and biological diversity. Agriculture 2025, 15, 927. [Google Scholar] [CrossRef] [Scilit]
- Zhao, Z.; Zhang, J.; Liu, R. Application of overground rock film mulching (ORFM) technology in Karst Rocky Desertification farmland: Improving soil moisture environment and crop root growth. Agronomy 2024, 14, 1265. [Google Scholar] [CrossRef] [Scilit]
- Xue, T.; Cheng, C.; Yang, F.; Zhang, L.; Xu, G.; Li, R.; Wang, J.; Zhang, L.; Liang, Z.; Zhou, J. Effect of organic mulching practices on soil properties in vineyards: A review. J. China Agric. Univ. 2024, 29, 206–218. [Google Scholar] [CrossRef]
- Zhang, H.; Yu, S.; Lv, W.; Wang, X.; Lu, P.; Zhang, H.; Zhang, J.; Bai, N.; Xu, C.; Zhu, X.; et al. Biodegradable mulch films divergently regulate soil carbon cycle by reshaping microbial communities and functional genes. J. Hazard. Mater. 2026, 506, 141616. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ji, M.; Li, L.; Xu, J.; Gao, L.; Liu, H.; Yao, Y.; Niu, G.; Zhang, L.; Hao, B. Mulching with orchard pruning branches exerts positive effects on improving the soil micro-ecological environment and enhancing fruit quality. Plant Soil 2026. [Google Scholar] [CrossRef] [Scilit]
- Ghani, A.; Dexter, M.; Perrott, K.W. Hot-water extractable carbon in soils: A sensitive measurement for determining impacts of fertilisation, grazing and cultivation. Soil Biol. Biochem. 2003, 35, 1231–1243. [Google Scholar] [CrossRef] [Scilit]
- Blair, G.J.; Lefroy, R.D.B.; Lisle, L. Soil carbon fractions based on their degree of oxidation, and the development of a carbon management index for agricultural systems. Aust. J. Agric. Res. 1995, 46, 1459–1466. [Google Scholar] [CrossRef] [Scilit]
- Cambardella, C.A.; Elliott, E. Particulate soil organic-matter changes across a grassland cultivation sequence. Soil Sci. Soc. Am. J. 1992, 56, 777–783. [Google Scholar] [CrossRef] [Scilit]
- Heanes, D.L. Determination of total organic-C in soils by an improved chromic acid digestion and spectrophotometric procedure. Commun. Soil Sci. Plant Anal. 1984, 15, 1191–1213. [Google Scholar] [CrossRef] [Scilit]
- Motsi, H.; Clarke, C.E.; Hardie, A.G.; Francis, M.L.; Potts, A.J. Comparison of alternative chemical density and physical methods for isolating soil organic matter fractions in high carbon soils. CATENA 2026, 264, 109788. [Google Scholar] [CrossRef] [Scilit]
- Vance, E.D.; Brookes, P.C.; Jenkinson, D.S. Microbial biomass measurements in forest soils: The use of the chloroform fumigation-incubation method in strongly acid soils. Soil Biol. Biochem. 1987, 19, 697–702. [Google Scholar] [CrossRef] [Scilit]
- Menzel, P.; Ng, K.L.; Krogh, A. Fast and sensitive taxonomic classification for metagenomics with Kaiju. Nat. Commun. 2016, 7, 11257. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhu, W.; Lomsadze, A.; Borodovsky, M. Ab initio gene identification in metagenomic sequences. Nucleic Acids Res. 2010, 38, e132. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, S.; Zhou, Y.; Chen, Y.; Gu, J. fastp: An ultra-fast all-in-one FASTQ preprocessor. Bioinformatics 2018, 34, i884–i890. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fu, L.; Niu, B.; Zhu, Z.; Wu, S.; Li, W. CD-HIT: Accelerated for clustering the next-generation sequencing data. Bioinformatics 2012, 28, 3150–3152. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Langmead, B.; Salzberg, S.L. Fast gapped-read alignment with Bowtie 2. Nat. Methods 2012, 9, 357–359. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hong, C.; Manimaran, S.; Shen, Y.; Perez-Rogers, J.F.; Byrd, A.L.; Castro-Nallar, E.; Crandall, K.A.; Johnson, W.E. PathoScope 2.0: A complete computational framework for strain identification in environmental or clinical sequencing samples. Microbiome 2014, 2, 33. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Qin, J.; Li, Y.; Cai, Z.; Li, S.; Zhu, J.; Zhang, F.; Liang, S.; Zhang, W.; Guan, Y.; Shen, D.; et al. A metagenome-wide association study of gut microbiota in type 2 diabetes. Nature 2012, 490, 55–60. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Shi, C.H.; Wang, X.Q.; Jiang, S.; Zhang, L.Q.; Luo, J. Revealing the role of the rhizosphere microbiota in reproductive growth for fruit productivity when inorganic fertilizer is partially replaced by organic fertilizer in pear orchard fields. Microb. Biotechnol. 2023, 16, 1373–1392. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xu, M.; Lou, Y.; Sun, X.; Wang, W.; Baniyamuddin, M.; Zhao, K. Soil organic carbon active fractions as early indicators for total carbon change under straw incorporation. Biol. Fertil. Soils 2011, 47, 745–752. [Google Scholar] [CrossRef] [Scilit]
- Biederbeck, V.; Janzen, H.; Campbell, C.; Zentner, R. Labile soil organic matter as influenced by cropping practices in an arid environment. Soil Biol. Biochem. 1994, 26, 1647–1656. [Google Scholar] [CrossRef] [Scilit]
- Wendling, B.; Jucksch, I.; Mendonca, E.; Alvarenga, R. Organic-matter pools of soil under pines and annual cultures. Commun. Soil Sci. Plant Anal. 2010, 41, 1707–1722. [Google Scholar] [CrossRef] [Scilit]
- Puget, P.; Drinkwater, L.E. Short-term dynamics of root-and shoot-derived carbon from a leguminous green manure. Soil Sci. Soc. Am. J. 2001, 65, 771–779. [Google Scholar] [CrossRef] [Scilit]
- Purakayastha, T.; Rudrappa, L.; Singh, D.; Swarup, A.; Bhadraray, S. Long-term impact of fertilizers on soil organic carbon pools and sequestration rates in maize–wheat–cowpea cropping system. Geoderma 2008, 144, 370–378. [Google Scholar] [CrossRef] [Scilit]
- Hassan, W.; Bashir, S.; Ahmed, N.; Tanveer, M.; Shah, A.N.; Bano, R.; David, J. Labile organic carbon fractions, regulator of CO2 emission: Effect of plant residues and water regimes. Clean–Soil Air Water 2016, 44, 1358–1367. [Google Scholar] [CrossRef] [Scilit]
- Campbell, B.J.; Polson, S.W.; Hanson, T.E.; Mack, M.C.; Schuur, E.A. The effect of nutrient deposition on bacterial communities in Arctic tundra soil. Environ. Microbiol. 2010, 12, 1842–1854. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Das, B.; Chakraborty, D.; Singh, V.; Aggarwal, P.; Singh, R.; Dwivedi, B.; Mishra, R. Effect of integrated nutrient management practice on soil aggregate properties, its stability and aggregate-associated carbon content in an intensive rice–wheat system. Soil Tillage Res. 2014, 136, 9–18. [Google Scholar] [CrossRef] [Scilit]
- Yang, F.; Tang, J.; Yang, D.; Yang, T.; Liu, H.; Luo, W.; Wu, J.; Jianqiang, W.; Wang, L. Jasmonoyl-l-isoleucine and allene oxide cyclase-derived jasmonates differently regulate gibberellin metabolism in herbivory-induced inhibition of plant growth. Plant Sci. Int. J. Exp. Plant Biol. 2020, 300, 110627. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Guo, X.; Rossel, R.A.V.; Wang, G.; Xiao, L.; Wang, M.; Zhang, S.; Luo, Z. Particulate and mineral-associated organic carbon turnover revealed by modelling their long-term dynamics. Soil Biol. Biochem. 2022, 173, 108780. [Google Scholar] [CrossRef] [Scilit]
- Yuan, Z.; Jin, H.; Wang, Q.; Wu, Q.; Li, G.; Jin, X.; Ma, Q. Profile distributions of soil organic carbon fractions in a permafrost region of the Qinghai–Tibet Plateau. Permafr. Periglac. Process. 2020, 31, 538–547. [Google Scholar] [CrossRef] [Scilit]
- Zhang, X.; Wang, M.; Zhang, D.; Zhang, Y.; Wang, X. Increasing soil organic carbon pools and wheat yields by optimising tillage and fertilisation on the Loess Plateau in China. Eur. J. Soil Sci. 2022, 73, e13197. [Google Scholar] [CrossRef] [Scilit]
- Rodrigo, E.; Litskas, V.D.; Mairata, A.; Martínez Vidaurre, J.M.; Pou, A. Effect of organic mulches in vineyards: CH4 and N2O emissions and their contribution to the GWP and carbon balance. Front. Environ. Sci. 2026, 14, 1846259. [Google Scholar] [CrossRef] [Scilit]
- Duan, X.; Yan, Y.; Han, X.; Wang, Y.; Li, R.; Gao, F.; Zhang, L.; Wei, R.; Li, H.; Wang, H. Effects of biodegradable liquid film on the soil and fruit quality of Vitis Franco-american L. Hutai-8 berries. Horticulturae 2022, 8, 418. [Google Scholar] [CrossRef] [Scilit]
- Mairata, A.; Labarga, D.; Puelles, M.; Rivacoba, L.; Martin, I.; Portu, J.; Pou, A. Impact of organic mulches on grapevine health, growth and grape composition in nutrient-poor vineyard soils. OENO One 2024, 58, 4. [Google Scholar] [CrossRef] [Scilit]
- Fahey, T.J.; Heinz, A.K.; Mathisson, R.; Fahey, C.; Yavitt, J.B. How Much Soil Carbon is Derived from Woody Detritus? A Ten-Year Study of 13C Incorporation into Soil Organic Matter. Ecosystems 2024, 27, 867–878. [Google Scholar] [CrossRef] [Scilit]
- Xue, T.; Han, X.; Zhang, H.; Wang, Y.; Wang, H.; Li, H. Effects of a biodegradable liquid film on winter chill protection of winegrape cultivars. Sci. Hortic. 2019, 246, 398–406. [Google Scholar] [CrossRef] [Scilit]
- Zhang, X.; Lu, S.; Wang, C.; Zhang, A.; Wang, X. Optimization of tillage rotation and fertilization increased the soil organic carbon pool and crop yield in a semiarid region. Land Degrad. Dev. 2021, 32, 5241–5252. [Google Scholar] [CrossRef] [Scilit]
- Ferrando, L.; Rariz, G.; Martínez-Pereyra, A.; Fernández-Scavino, A. Endophytic diazotrophic communities from rice roots are diverse and weakly associated with soil diazotrophic community composition and soil properties. J. Appl. Microbiol. 2024, 135, lxae157. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, H.; Yang, S.; Semenov, M.V.; Yao, F.; Ye, J.; Bu, R.; Ma, R.; Lin, J.; Kurganova, I.; Wang, X.; et al. Temperature sensitivity of SOM decomposition is linked with a K-selected microbial community. Glob. Change Biol. 2021, 27, 2763–2779. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mbuthia, L.W.; Acosta-Martínez, V.; DeBruyn, J.; Schaeffer, S.; Tyler, D.; Odoi, E.; Mpheshea, M.; Walker, F.; Eash, N. Long term tillage, cover crop, and fertilization effects on microbial community structure, activity: Implications for soil quality. Soil Biol. Biochem. 2015, 89, 24–34. [Google Scholar] [CrossRef] [Scilit]
- Zhang, H.; Chen, M.Q.; Qiao, R.Q.; Ding, F.; Feng, H.; Jiang, R. Agronomic performances of biodegradable and non-biodegradable plastic film mulching on a maize cropping system in the semi-arid Loess Plateau, China. Pedosphere 2024, 34, 88–96. [Google Scholar] [CrossRef] [Scilit]
- Xiong, X.; Wang, P.; Zhao, Z.; Wang, J.; Liu, S.; Mei, F.; Wang, W.; Wang, Y.; Fang, X.; Zhu, Y.; et al. Can biodegradable film replace polyethylene film to obtain similar mulching effects on soil functions and maize productivity in irrigation region? A three-year experimental appraisal. J. Clean. Prod. 2025, 486, 144473. [Google Scholar] [CrossRef] [Scilit]
- Taguas, E.V.; Marin-Moreno, V.; Diez, C.M.; Mateos, L.; Barranco, D.; Mesas-Carrascosa, F.J.; Perez, R.; Garcia-Ferrer, A.; Quero, J.L. Opportunities of super high-density olive orchard to improve soil quality: Management guidelines for application of pruning residues. J. Environ. Manag. 2021, 293, 112785. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Manzoni, S.; Čapek, P.; Mooshammer, M.; Lindahl, B.D.; Richter, A.; Santrůčková, H. Optimal metabolic regulation along resource stoichiometry gradients. Ecol. Lett. 2017, 20, 1182–1191. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chaves, B.; Redin, M.; Giacomini, S.J.; Schmatz, R.; Léonard, J.; Ferchaud, F.; Recous, S. The combination of residue quality, residue placement and soil mineral N content drives C and N dynamics by modifying N availability to microbial decomposers. Soil Biol. Biochem. 2021, 163, 108434. [Google Scholar] [CrossRef] [Scilit]
- Mooshammer, M.; Wanek, W.; Hämmerle, I.; Fuchslueger, L.; Hofhansl, F.; Knoltsch, A.; Schnecker, J.; Takriti, M.; Watzka, M.; Wild, B.; et al. Adjustment of microbial nitrogen use efficiency to carbon:nitrogen imbalances regulates soil nitrogen cycling. Nat. Commun. 2014, 5, 3694. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mooshammer, M.; Wanek, W.; Zechmeister-Boltenstern, S.; Richter, A. Stoichiometric imbalances between terrestrial decomposer communities and their resources: Mechanisms and implications of microbial adaptations to their resources. Front. Microbiol. 2014, 5, 22. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Phukongchai, W.; Kaewpradit, W.; Rasche, F. Enhanced Nitrogen Release from Sugarcane Straw in a Sandy Soil Via Microbial Inoculants Efficient in Decomposing High C/N Ratio Organic Matter. J. Soil Sci. Plant Nutr. 2025, 25, 4385–4396. [Google Scholar] [CrossRef] [Scilit]
- Wang, X.; He, P.; Xu, X.; Qiu, S.; Zhao, S. Characteristics of rice straw decomposition and bacterial community succession for 2 consecutive years in a paddy field in southeastern China. Sci. Rep. 2022, 12, 20893. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mastný, J.; Bárta, J.; Kaštovská, E.; Picek, T. Decomposition of peatland DOC affected by root exudates is driven by specific r and K strategic bacterial taxa. Sci. Rep. 2021, 11, 18677. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tiwari, R.; Kumar, K.; Singh, S.; Nain, L.; Shukla, P. Molecular Detection and Environment-Specific Diversity of Glycosyl Hydrolase Family 1 β-Glucosidase in Different Habitats. Front. Microbiol. 2016, 7, 1597. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Rui, J.; Li, J.; Wang, S.; An, J.; Liu, W.T.; Lin, Q.; Yang, Y.; He, Z.; Li, X. Responses of Bacterial Communities to Simulated Climate Changes in Alpine Meadow Soil of the Qinghai-Tibet Plateau. Appl. Environ. Microbiol. 2015, 81, 6070–6077. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Malik, A.A.; Martiny, J.B.H.; Brodie, E.L.; Martiny, A.C.; Treseder, K.K.; Allison, S.D. Defining trait-based microbial strategies with consequences for soil carbon cycling under climate change. ISME J. 2020, 14, 1–9. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Roller, B.R.; Schmidt, T.M. The physiology and ecological implications of efficient growth. ISME J. 2015, 9, 1481–1487. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Averill, C. Divergence in plant and microbial allocation strategies explains continental patterns in microbial allocation and biogeochemical fluxes. Ecol. Lett. 2014, 17, 1202–1210. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Soong, J.L.; Fuchslueger, L.; Marañon-Jimenez, S.; Torn, M.S.; Janssens, I.A.; Penuelas, J.; Richter, A. Microbial carbon limitation: The need for integrating microorganisms into our understanding of ecosystem carbon cycling. Glob. Change Biol. 2020, 26, 1953–1961. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Manzoni, S.; Porporato, A. Soil carbon and nitrogen mineralization: Theory and models across scales. Soil Biol. Biochem. 2009, 41, 1355–1379. [Google Scholar] [CrossRef] [Scilit]
- Billings, S.A.; Ziegler, S.E. Altered patterns of soil carbon substrate usage and heterotrophic respiration in a pine forest with elevated CO2 and N fertilization. Glob. Change Biol. 2008, 14, 1025–1036. [Google Scholar] [CrossRef] [Scilit]
- Carney, K.M.; Hungate, B.A.; Drake, B.G.; Megonigal, J.P. Altered soil microbial community at elevated CO2 leads to loss of soil carbon. Proc. Natl. Acad. Sci. USA 2007, 104, 4990–4995. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yang, C.; Zhang, N.; Zhao, F.; Wang, J. Mulching practices decreased soil microbial carbon degradation potential under spring maize in the Loess Plateau of China. Agric. Ecosyst. Environ. 2025, 381, 109465. [Google Scholar] [CrossRef] [Scilit]
- Fierer, N. Embracing the unknown: Disentangling the complexities of the soil microbiome. Nat. Rev. Microbiol. 2017, 15, 579–590. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Contesini, F.J.; de Alencar Figueira, J.; Kawaguti, H.Y.; de Barros Fernandes, P.C.; de Oliveira Carvalho, P.; da Graça Nascimento, M.; Sato, H.H. Potential applications of carbohydrases immobilization in the food industry. Int. J. Mol. Sci. 2013, 14, 1335–1369. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tan, H.; Barret, M.; Mooij, M.J.; Rice, O.; Morrissey, J.P.; Dobson, A.; Griffiths, B.; O’Gara, F. Long-term phosphorus fertilisation increased the diversity of the total bacterial community and the phoD phosphorus mineraliser group in pasture soils. Biol. Fertil. Soils 2013, 49, 661–672. [Google Scholar] [CrossRef] [Scilit]
- Tu, Q.; He, Z.; Wu, L.; Xue, K.; Xie, G.; Chain, P.; Reich, P.B.; Hobbie, S.E.; Zhou, J. Metagenomic reconstruction of nitrogen cycling pathways in a CO2-enriched grassland ecosystem. Soil Biol. Biochem. 2017, 106, 99–108. [Google Scholar] [CrossRef] [Scilit]
- Zhong, Y.; Yan, W.; Wang, R.; Wang, W.; Shangguan, Z. Decreased occurrence of carbon cycle functions in microbial communities along with long-term secondary succession. Soil Biol. Biochem. 2018, 123, 207–217. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.