


Abstract
Microbial inoculants are widely used to improve the fermentation and aerobic stability of silages, particularly in sorghum, which is susceptible to deterioration; therefore, this study evaluated the effects of Lentilactobacillus buchneri (Lb), alone or combined with Lentilactobacillus hilgardii (Lb + Lh), on the fermentation profile, microbial stability, chemical composition, and aerobic stability of whole-plant sorghum silage. A completely randomized design was adopted in a 3 × 3 factorial scheme, with three fermentation periods (20, 60 and 100 days) and three microbial inoculants (control, Lb and Lb + Lh), with five replicates per factorial treatment; the fermentation parameters, chemical composition, microbial populations, and aerobic stability were evaluated. A interaction (p < 0.05) between inoculants and fermentation periods was observed for pH, organic acids, microbial counts, and aerobic stability; inoculated silages showed increased lactic acid bacteria, higher acetic and propionic acid production, and inhibition of yeasts and molds, especially at 100 days, resulting in improved aerobic stability at 60 and 100 days. The microbial diversity was lower in inoculated factorial treatments, with predominance of Lentilactobacillus, while the control showed a higher abundance of undesirable microorganisms; Kazachstania was the predominant fungal genus. In conclusion, inoculation improves the fermentation quality, microbial stability, and aerobic stability of sorghum silage, reducing losses.
1. Introduction
Forage scarcity during dry spells in arid and semi-arid regions hampers livestock productivity, but ensiling offers a solution by preserving crops like sorghum, which thrives in dry environments with lower water needs compared to the traditional use of corn [1]. Ensiling ensures a steady feed supply throughout the year and mitigates the effects of drought through the storage of forage in an anaerobic, acidic, and stable environment [2]. However, spoilage often occurs when the silo is opened, as exposure to air promotes the growth of yeasts and molds, which, in turn, rapidly consume the lactic acid, raising the pH and compromising the silage’s preservation [3,4]. Therefore, aerobic stability is of high concern for silages made in tropical countries because the warm and humid climate can accelerate spoilage, leading to nutrient losses and reduced feed quality [5,6,7].
To address this issue, the use of microbial inoculants, particularly those made of heterofermentative lactic acid bacteria (LAB), such as Lentilactobacillus buchneri and Lentilactobacillus parabuchneri, can produce acetic acid (AA), propionic acid (PA) and 1,2-propanediol, whose strong antifungal activity enhances aerobic stability [3,4]. However, the AA production rate varies between species and even among strains. The efficacy of Lentilactobacillus buchneri in producing AA becomes more pronounced after 45 to 60 days of fermentation, achieving concentrations sufficient to ensure aerobic stability. In contrast, Lentilactobacillus hilgardii demonstrates a significantly earlier onset of AA production, typically peaking within 15 to 30 days of fermentation, a characteristic particularly relevant for semi-arid regions, where early silo opening is common due to forage scarcity, contributing to reduced losses during drought periods [8,9,10].
Sorghum silages without additives often have low aerobic stability, leading to nutrient losses during both anaerobic fermentation and the aerobic phase after silo opening, and while sorghum is suitable for ensiling due to its high content of water-soluble carbohydrates (WSCs) that drive intense fermentations and a sharp pH drop from lactic acid production, the excessive WSCs may surpass the fermentation capacity of LAB, leaving residual sugars in the silage [4,11]. The most common fungal spoilage occurs after the silo is opened and the silage is exposed to air, but residual carbohydrates in sorghum silage can also promote the growth of yeasts and molds during anaerobiosis, triggering a secondary fermentation process alongside the primary LAB metabolism, where these yeasts convert sugars into alcohol and carbon dioxide, causing significant dry matter (DM) losses and reducing the silage’s net energy value even before the silo is opened [11,12]. Similar anaerobic deterioration processes have also been observed in other high-sugar forages, such as sugarcane silage, due to its high sucrose content [13,14].
In light of this, we hypothesize that inoculating whole-plant sorghum silage with a combination of L. hilgardii and L. buchneri promotes the rapid growth of heterofermentative LAB and the production of antifungal compounds, particularly acetic acid, thereby modifying bacterial and fungal communities, reducing alcoholic fermentation, and improving aerobic stability even after a short fermentation period. This approach may allow for the use of the silage without compromising its nutritional quality or aerobic stability compared to the traditional standalone L. buchneri inoculation.
This study aimed to evaluate the effects of inoculating whole-plant sorghum silages with L. buchneri, either alone or in combination with L. hilgardii, on the fermentation profile, bacterial and fungal succession, chemical composition, dry matter losses, and aerobic stability of silages ensiled for fermentation periods.
2. Materials and Methods
2.1. Location, Ensiling and Experiment
Sorghum [Sorghum bicolor (L.) Moench cv. BRS Ponta Negra] was cultivated using a manual seeder (Krupp Seeder®, São Leopoldo, RS, Brazil) at a depth of ±2 cm and spaced 0.20 × 0.80 m, with five seeds per linear meter after the soil had been ploughed and harrowed in March 2023 in Riachão, Paraíba, Brazil, located at latitude south 06°32′25″ and longitude west 35°39′35″, with an average altitude of ±175 m. Simple superphosphate at 100 kg/ha (Heringer Fertilizers®, São Paulo, SP, Brazil) and urea topdressing at 45 kg N/ha (Heringer Fertilizers®, São Paulo, SP, Brazil) were applied as chemical fertilizers. Sorghum was manually harvested around 110 days of age and transported to the Forage Laboratory of the Federal University of Paraíba (UFPB), Areia, Paraíba, Brazil, located at latitude south 6°58′12″, longitude west 35°42′15″, and ±619 m altitude, to be chopped (±10 mm) using a stationary machine (EN9-F3B, Nogueira®, Itapira, SP, Brazil), stored in bucket silos (55 cm diameter × 19 cm height, 4 L) (630EE, GrouPack®, Cabedelo, PB, Brazil), compacted (density of ±600 kg/m3), tape-sealed, weighed, and stored at room temperature.
The completely randomized design was arranged in a 3 × 3 factorial scheme (n = 45), with three opening periods (D20, D60, and D100), and three additives: inoculated with L. buchneri (Lb) (Lallemand®, Aparecida de Goiânia, GO, Brazil), inoculated with a combination of L. hilgardii CNCM I-4785 and L. buchneri NCIMB-40788 (Lb + Lh) (Lallemand®, Aparecida de Goiânia, GO, Brazil) and a control group. The microbial inoculants were sprayed according to the manufacturer’s recommendation [3 × 10⁵ CFU/g of forage (1 g/t of forage)] and diluted in 50 mL distilled water, and both the inoculants and water (control group) were applied on individual 5 kg sorghum piles before silo compaction.
Fresh sorghum samples were collected at ensiling, and silage samples were taken at each opening period. Samples (25 g) were homogenized in 225 mL of 0.85% NaCl saline solution using an industrial blender (LAR.2, METVISA®, Brusque, SC, Brazil) for 1 min. The resulting aqueous extract was then filtered through sterile cotton gauze, divided into 3 aliquots for the subsequent analyses.
2.2. Bromatological and Chemical Analyses
Samples were partially dried in a forced-air circulation oven (55 °C/72 h) and ground in a mill (Wiley®, Arthur H. Thomas, Philadelphia, PA, USA) with a 1 mm sieve (Table 1). The bromatological analyses followed DM (method 934.01), fresh matter (FM) (method 972.43), ash (method 942.05), and crude protein (CP) (N × 6.25, method 984.13) determination, according to the AOAC [15]. The samples were also analyzed for neutral detergent fiber (NDFam) using thermostable α-amylase without sodium sulfite [16].
Table 1.
Chemical compositions and microbial populations of BRS Ponta Negra forage sorghum with application of microbial additives before ensiling.
The pH was measured using a digital potentiometer (K39-1420A, KASVI®, São José dos Pinhais, PR, Brazil), while a 50 mL aliquot of the aqueous extract was acidified with H2SO4 (1:1 v/v, Neon®, Suzano, SP, Brazil) for ammonia nitrogen (NH3-N) quantification following [17], and the levels of WSCs were determined using the phenol–sulfuric acid method as described in [18].
2.3. Organic Acid Quantification
A 10 mL aliquot of the aqueous extract was acidified (H2SO4 1:1 v/v, Neon®, Suzano, SP, Brazil) and transferred to screw-cap test tubes (AJ03, PlenaLab®, Jundiaí, SP, Brazil), vortexed (Vortex Mixer VX-200, LabNet®, Edison, NJ, USA), and then 2 mL of metaphosphoric acid (Neon®, Suzano, SP, Brazil) was added. The solution was centrifuged (Mikro-120, Hettich Zentrifugen®, Tuttlingen, Germany) for 15 min at 13,000× g.
The supernatant was collected, stored in labeled and sealed 1.5 mL microtubes (CralPlast®, Cotia, SP, Brazil), and properly labeled, sealed, and stored under freezing conditions until analysis. Organic acids [lactic acid (LA), acetic acid (AA), propionic acid (PA), and butyric acid (BA)] were quantified by high-performance liquid chromatography (HPLC) (Shimadzu, SPD-10A VP, Kyoto, Japan) at the Animal Nutrition and Soils Laboratory of the Federal University of Piauí (UFPI), following the method of Siegfried et al. (1984) [19].
Chromatographic separation was performed using an Aminex HPX-87H column (Bio-Rad Laboratories, Hercules, CA, USA), with 0.005 M H2SO4 as the mobile phase, at a flow rate of 0.6 mL/min. Detection was carried out using a UV detector set at 210 nm, with an injection volume of 20 µ.
2.4. Microbial Culture and Identification
Serial dilutions from 101 to 108 were prepared and plated using the pour-plate method on 90 × 15 mm sterile Petri dishes (FirstLab®, São José dos Pinhais, PR, Brazil). MRS agar (De Man, Rogosa & Sharpe, K25-1043, Kasvi®, São José dos Pinhais, PR, Brazil) at 37 °C/48 h was used for LAB cultivation, while DRBC agar (Dicloran Rose Bengal Chloramphenicol, Oxoid™, Basingstoke, UK) at 25 °C/72 h and 25 °C/120 h was used for yeast and mold cultivation, respectively. Colony-forming units (CFUs) were counted on plates containing 25 to 250 CFUs [20].
2.5. Aerobic Stability and Dry Matter Loss Assessment
Silage (1 kg) was collected at the time of opening, weighed, and returned to its respective bucket without compaction, and the samples were then exposed for 144 h in a room with controlled temperature (±25 °C). A data logger (AK285 New, AKSO®, São Leopoldo, RS, Brazil) was placed in the center of each silo to record the temperature every 10 min, while three additional loggers measured the ambient temperature in the room. Aerobic stability was defined as the number of hours the silage remained stable, with deterioration starting when the internal temperature of the silage rose two degrees Celsius above the ambient temperature [21].
DM losses (DML) were calculated by subtracting the final bucket weight from the initial weight, expressed as a percentage of the initial weight, using the equation from [22]:
where DML (g DM/kg FM) is the dry matter losses in grams per kilogram of fresh matter; DMop is the kg of dry matter at silo opening (silage amount in kg × % DM); DMcl is the kg of dry matter at silo closure (forage amount in kg × % DM).
DML (g DM/kg FM) = 1000 − [(DMop/DMcl) × 1000]
2.6. DNA Extraction and Marker Gene Sequencing
Macerated silages (25 g) were homogenized in 225 mL of PBS, filtered through sterile gauze, and centrifuged at 6000× g for 4 min at 4 °C, with the supernatant discarded. The pellet was washed with PBS, resuspended in 900 µL of PBS, and stored at −20 °C for molecular analyses. Bacterial DNA was extracted using the ZymoBIOMICS DNA Miniprep Kit (Zymo Research, Irvine, CA, USA) following the manufacturer’s instructions. Libraries were prepared using primers targeting the V3–V4 region of the 16S rRNA (~470 bp, amplified with primers 341F × 806R) for bacterial studies, with primer sequences 341F: 5′-CCTAYGGGRBGCASCAG-3′ and 806R: 5′-GGACTACNNGGGTATCTAAT-3′. For fungal sequencing, libraries were prepared using primers targeting the ITS region (~380 bp, amplified with primers ITS5-1737F × ITS2-2043R), with primer sequences ITS5-1737F: 5′-GGAAGTAAAAGTCGTAACAAGG-3′ and ITS2-2043R: 5′-GCTCGTTCTTCATCGATGC-3′. The final library concentration was achieved by loading 6 pM into the flow cell, with 15% PhiX added for diversity comparison. Sequencing was performed on an Illumina MiSeq, with bacterial and fungal amplicons sequenced using the Illumina platform (paired-end 250 bp), generating 50–100 million raw reads per sample for each.
2.7. Bioinformatics
The demultiplexed raw fastq files were imported into QIIME2 v. 2023.9, and DADA2 was used to denoise low-quality reads and call the Amplicon Sequence Variants (ASVs), applying a length truncation of 240 bp for 16S rRNA amplicons and no truncation for ITS [23,24].
A Naïve Bayes classifier algorithm, based on the Genome Taxonomy Database (GTDB) v. 20.7.0, was used for the V3-V4 hypervariable regions of the 16S rRNA gene, whereas the UNITE database v. 9.0 with 99% similarity was used for the bacterial and fungal taxonomic classification, with ASVs classified as host DNA, such as Chloroplasts and Mitochondria, excluded from the study [25,26].
Samples were normalized to 19,750 and 37,000 reads per sample for bacterial and fungal studies, respectively. Figures were plotted in R v. 4.1.3 using the ggplot2, phyloseq, and microbiomeR packages, with alpha diversity analysis involving the calculation of observed features (transformed to log10), along with Shannon and Simpson indices, while non-metric multidimensional scaling (NMDS) was used to visualize the Bray–Curtis dissimilarity matrix’s distances between samples, which were further used for beta diversity analysis [27,28,29].
2.8. Statistical Analyses
The Shapiro–Wilk test was used to assess the normality and homogeneity of variances. Following this, a two-way factorial ANOVA with interaction effects was applied to examine the influence of two independent factors (fermentation period and inoculant) on the dependent variable (sorghum fermentation quality), while also considering the interaction between these factors, according to the following model:
where Yỉʝκ is the response variable; µ is the overall mean; FPỉ is the fixed effect of the fermentation i period; Iʝ is the fixed effect of the j inoculant; (FP*I)ỉʝ is the interaction effect between the fermentation period and inoculant; ℮ỉʝk is the random experimental error.
Yỉʝκ = µ + FPỉ + Iʝ + (FP*I)ỉʝ + ℮ỉʝκ
When significant effects were found for the fermentation period, inoculant, or their interaction, a post hoc Tukey test was performed to compare the means at a 5% significance level, using Sisvar® software version 5.6 [30].
The statistical differences in the alpha diversity indices were assessed using the non-parametric Kruskal–Wallis test for group comparisons and the Wilcoxon Mann–Whitney rank sum test for pairwise comparisons. Permutational Multivariate Analysis of Variance (PERMANOVA) was used to test for differences in the beta diversity between experimental groups, and Principal Coordinates Analysis (PCoA) was used to visualize the dissimilarities among samples. Linear Discriminant Analysis Effect Size (LEfSe) was used to examine the differential abundance of specific genera between experimental groups, while differential predicted functions between experimental groups were calculated using the DESeq2 package [31,32]. Spearman correlation was applied to the abundance counts of Lentilactobacillus in the inoculated groups and Lactiplantibacillus, Levilactobacillus, and Secundilactobacillus in the control group with log10-transformed average pH and temperature values.
3. Results
3.1. Sorghum Silage Composition and Fermentation Profile
There was no interaction between the FP and I on the FM, ash, and NDF (Table 2). However, the DM and CP levels were influenced by the interaction effect (p < 0.001). The DM and CP were higher in the control, Lb, and Lb + Lh at days D20, D60, and D100, respectively, while the OM peaked at D60 and was higher in the control, and the ash content reached its highest in the Lb + Lh silage at D100 (Table 2). The WSCs, pH, ammonia nitrogen (NH3-N), and DML were affected by the interaction of the FP and I (Table 3). The pH had its peak value in the control at D20 and was the lowest in the Lb at D100. The WSC content peaked in the Lb at D20, while the NH3-N concentrations were the highest in the Lb + Lh at D60 and the Lb at D100 (Table 3). DML were the lowest in the Lb at D20 and the Lb + Lh at D100 (Table 3).
Table 2.
Chemical compositions of forage sorghum silages inoculated with Lentilactobacillus buchneri and Lentilactobacillus hilgardii stored for 20, 60, and 100 days.
Table 3.
Fermentation profiles and dry matter losses of forage sorghum silages inoculated with Lentilactobacillus buchneri and Lentilactobacillus hilgardii stored for 20, 60, and 100 days.
The highest LA concentrations were observed in the control at D20 and the Lb at D100, while the lowest one was in the control at D100 (Table 4). The AA concentrations were similar across factorial treatments at D20, while both the Lb and Lb + Lh had higher values than the control from D60 onwards (Table 4). PA and BA were higher in the Lb than in the control at D20 and D100 (Table 4).
Table 4.
Organic acid contents of forage sorghum silage inoculated with Lentilactobacillus buchneri and Lentilactobacillus hilgardii and stored for 20, 60, and 100 days.
The organic acid concentrations were influenced by the FP and I (p < 0.05). The FP showed that both AA and LA were the highest at D100, whereas PA was the highest at D20 (Table 4). The I showed that all organic acids were higher in the LB than in the other factorial treatments, but the LA/AA ratio was the lowest in the Lb + Lh (Table 4).
3.2. Bacteria, Yeast and Mol Culturing
The LAB counts were high in the Lb + Lh and Lb, while the control had the lowest counts at D20. At D60, the Lb + Lh maintained the highest counts, followed by the Lb and control (Table 5). By D100, the LAB counts dropped in absolute numbers across all factorial treatments, but the Lb + Lh remained with the top counts (Table 5).
Table 5.
Quantification of microbial populations of lactic acid bacteria (LAB), yeasts, and molds in forage sorghum silages inoculated with Lentilactobacillus buchneri and Lentilactobacillus hilgardii and stored for 20, 60, and 100 days.
An FP effect (p < 0.001) was observed for yeasts and molds. Yeast counts were the lowest at D60 and peaked at D100 (Table 5). Mold counts were high at D20 and D60 but dropped to zero by D100 (Table 5). The I effect showed the highest LAB counts in the Lb + Lh, with lower yeast counts in both the Lb + Lh and Lb (Table 5). No I effect was noted for molds.
3.3. Aerobic Stability Nutritive Value Loss
For maximum temperature, the control had the highest values across all periods, while both the Lb and Lb + Lh showed lower, comparable values (Table 6). For average temperature, the control silage reached higher values starting from D60, while the inoculated factorial treatments had lower average values (Table 6).
Table 6.
Aerobic stabilities of forage sorghum silages inoculated with Lentilactobacillus buchneri and Lentilactobacillus hilgardii stored for 20, 60, and 100 days.
The FP effect showed that, by D100, the aerobic stability decreased and both the average temperature and maximum temperature rose, while the minimum temperature increased from D60 onward (Table 6). The inoculant effect showed higher aerobic stability in the inoculated silages, while the control had higher maximum and average temperatures (Table 6). No inoculant effect was observed on the minimum temperature or time of maximum temperature.
3.4. Bacterial and Fungal Diversity Analyses
It was possible to retrieve 3997 and 1818 ASVs after the denoising step for the bacterial and fungal datasets, which was enough to cover the species diversity across all groups.
There was no significant difference in the alpha diversity indices across different silo opening periods for the bacterial communities, while the use of inoculants and their interaction effects were highly significant (p < 0.01) (Figure A1). The control group initially showed slight low values of bacterial richness and evenness at D20, but this pattern reversed at D60 and D100, with the control group exhibited significantly higher alpha diversity index values than both inoculated groups (Figure A1). Meanwhile, time and its interaction with inoculation had a significant effect (p < 0.01) on the fungal communities, while the use of inoculant alone showed no significant influence (Figure A2).
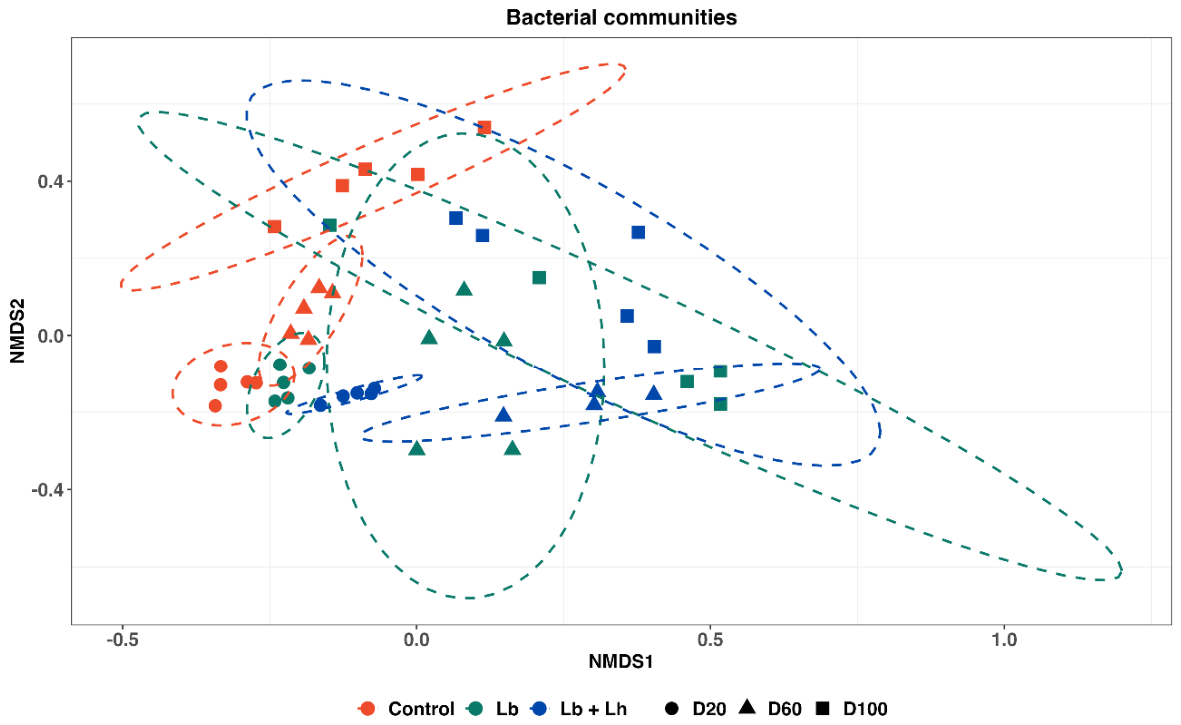
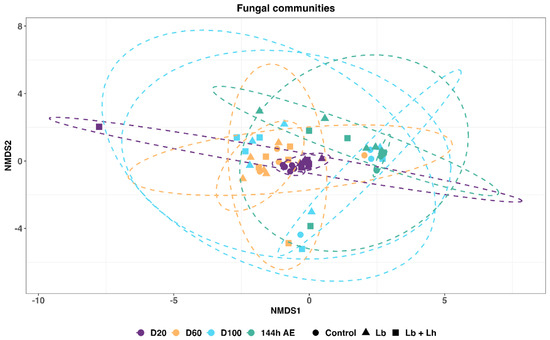
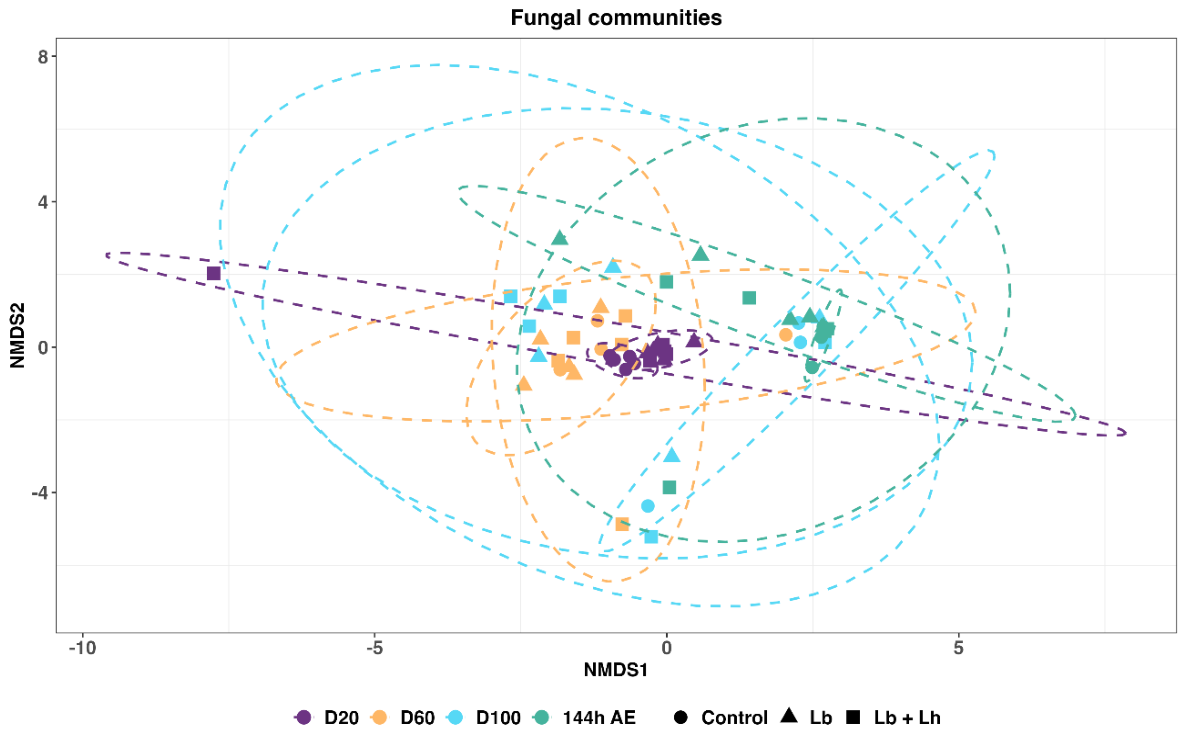
The beta diversity revealed distinctly different bacterial compositions among all groups, with both variables (time and inoculation) and their interaction being highly significant (p < 0.01). There were distinct cluster formations at D20, which drifted away progressively at D60 and D100, indicating increasing dispersion over time and dissimilarity, especially when comparing the inoculated groups to the control (Figure 1). The fungal communities showed higher dissimilarity between groups at D20, with higher dispersion and less evident cluster formation at D60, D100 and 144 h aerobic stability (Figure 2).
Figure 1.
Non-metric multidimensional scaling (NMDS) analysis based on Bray-Curtis distance matrix of bacterial communities in sorghum silages inoculated with microbial additives at 20, 60, and 100 days of fermentation. D20: sorghum forage silage after 20 days of fermentation; D60: sorghum forage silage after 60 days of fermentation; D100: inoculated sorghum forage silage after 100 days of fermentation. Control: untreated silage (without inoculant); Lb: Lentilactobacillus buchneri strain; Lb + Lh: Lentilactobacillus hilgardii CNCM I 4785 combined with L. buchneri NCIMB 40788.
Figure 2.
Non-metric multidimensional scaling (NMDS) analysis based on Bray-Curtis distance matrix of fungal communities in sorghum silages inoculated with microbial additives at 20, 60, and 100 days of fermentation and after 144 h of aerobic exposure. D20: sorghum forage silage after 20 days of fermentation; D60: sorghum forage silage after 60 days of fermentation; D100: inoculated sorghum forage silage after 100 days of fermentation; 144 h AE: silage exposed to air for 144 h. Control: untreated silage (without inoculant); Lb: Lentilactobacillus buchneri strain; Lb + Lh: Lentilactobacillus hilgardii CNCM I 4785 combined with L. buchneri NCIMB 40788.
The relative abundance chart showed Bacillota as the predominant bacterial phylum in all groups, with a progressive increase in the proportions of Pseudomonadota and Actinomycetota at D60 and D100 (Figure A3). The phyla Ascomycota and Basidiomycota were the main taxa in the fungal analysis (Figure A4).
The family Lactobacillaceae was the main driver of sorghum silage fermentation in all groups at D20 (Figure A5). Although the inoculated groups retained it as the main relative abundant family over time, the control group presented a surge in other taxa such as Micrococcaceae, Bacillaceae_D, Moraxellaceae, Staphylococcaceae, Clostridiaceae, Paenibacillaceae and Lachnospiraceae at D60 and D100 (Figure A5). The Saccharomycetaceae family was widely distributed across all groups, dominating the fungal composition at the family level, followed by Mycosphaerellaceae, Glomerellaceae, and Aspergillaceae, which were present in some samples (Figure A6).
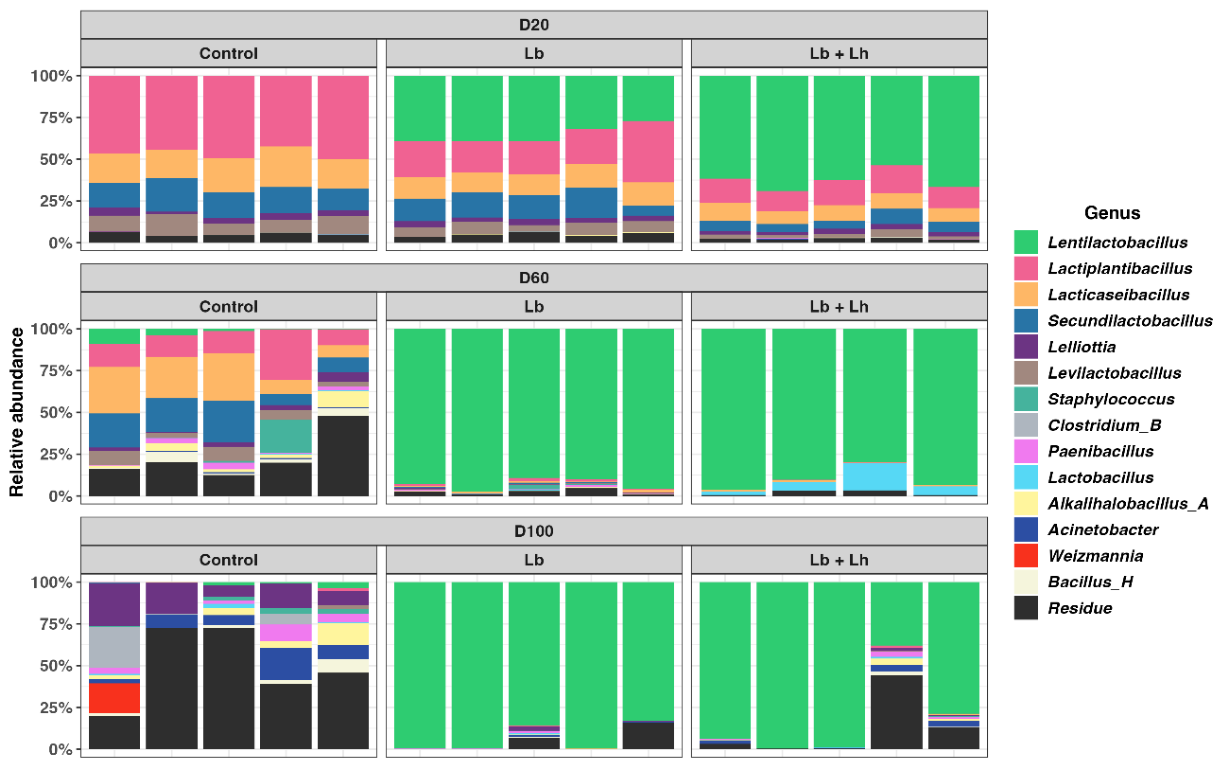
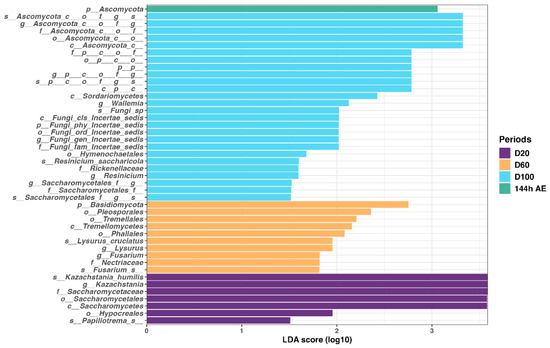
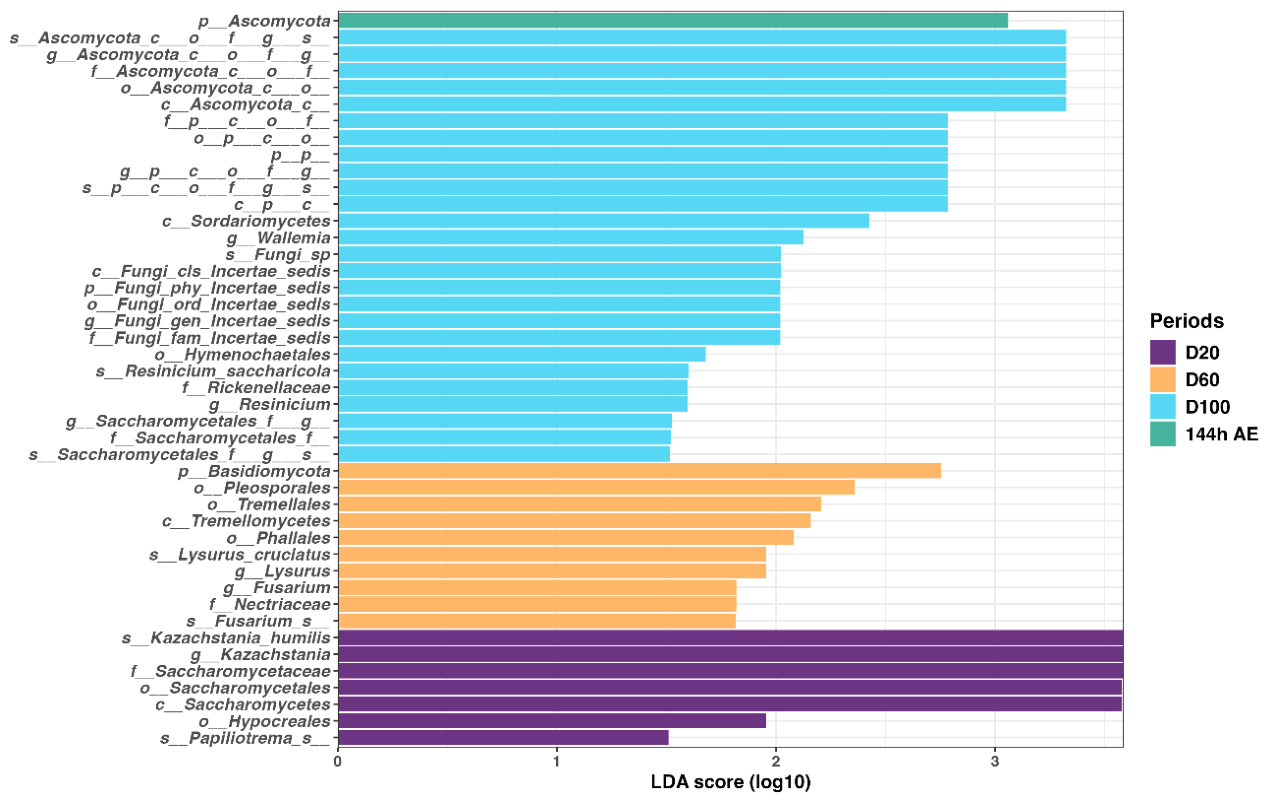
The fermentation pattern was also influenced by inoculation, as shown in the genus plot. Lentilactobacillus was the most prevalent genus at D20 for the Lb + Lh group and, to a lesser extent, the Lb group, while in the control group, it had no effect, and Lactiplantibacillus was the most abundant genus (Figure 3). The genera Lacticaseibacillus, Secundilactobacillus, and Levilactobacillus also played a role in fermentation during the initial stage (Figure 3). While the inoculated groups remained stable over time, the control group exhibited a microbial composition shift at D60, with increased relative abundances of Alkalihalobacillus A, Clostridium_B, Paenibacillus, and Staphylococcus, as well as a complete microbial inversion driven by clostridia and other non-LAB taxa, such as Lelliottia (Figure 3). Likewise, the differential abundance analysis showed the same pattern, with the dominance of communities at all opening times, while the control group showed non-LAB taxa taking over at D60 and D100 (Figure A7, Figure A8 and Figure A9). In line with the family pattern, the fungal communities exhibited less biodiversity at the genus level compared to the bacterial communities, with Kazachstania as the dominant taxon in all periods, including at the aerobic stability, while Aspergillus, Lysurus, Zasmidium, Pleosporales genus Incertae sedis, Colletotrichum, and Saccharomycetales genus Incertae sedis were present in smaller proportions across samples (Figure A10). The differential abundance showed an association of Kazachstania with the early fermentation stage, while low-abundant taxa like Wallemia, Fungi_phy_Incertae_sedis, and Lysurus were associated with later stages of fermentation (Figure 4).
Figure 3.
Relative abundances of bacterial genera in sorghum silages inoculated with microbial additives at 20, 60, and 100 days of fermentation. D20: sorghum forage silage after 20 days of fermentation; D60: sorghum forage silage after 60 days of fermentation; D100: inoculated sorghum forage silage after 100 days of fermentation. Control: untreated silage (without inoculant); Lb: Lentilactobacillus buchneri strain; Lb + Lh: Lentilactobacillus hilgardii CNCM I 4785 combined with L. buchneri NCIMB 40788.
Figure 4.
Differential fungal abundances in sorghum silages inoculated with microbial additives at 20, 60, and 100 days of fermentation and after 144 h of aerobic exposure. D20: sorghum forage silage after 20 days of fermentation; D60: sorghum forage silage after 60 days of fermentation; D100: inoculated sorghum forage silage after 100 days of fermentation; 144 h. AE: silage exposed to air for 144 h.
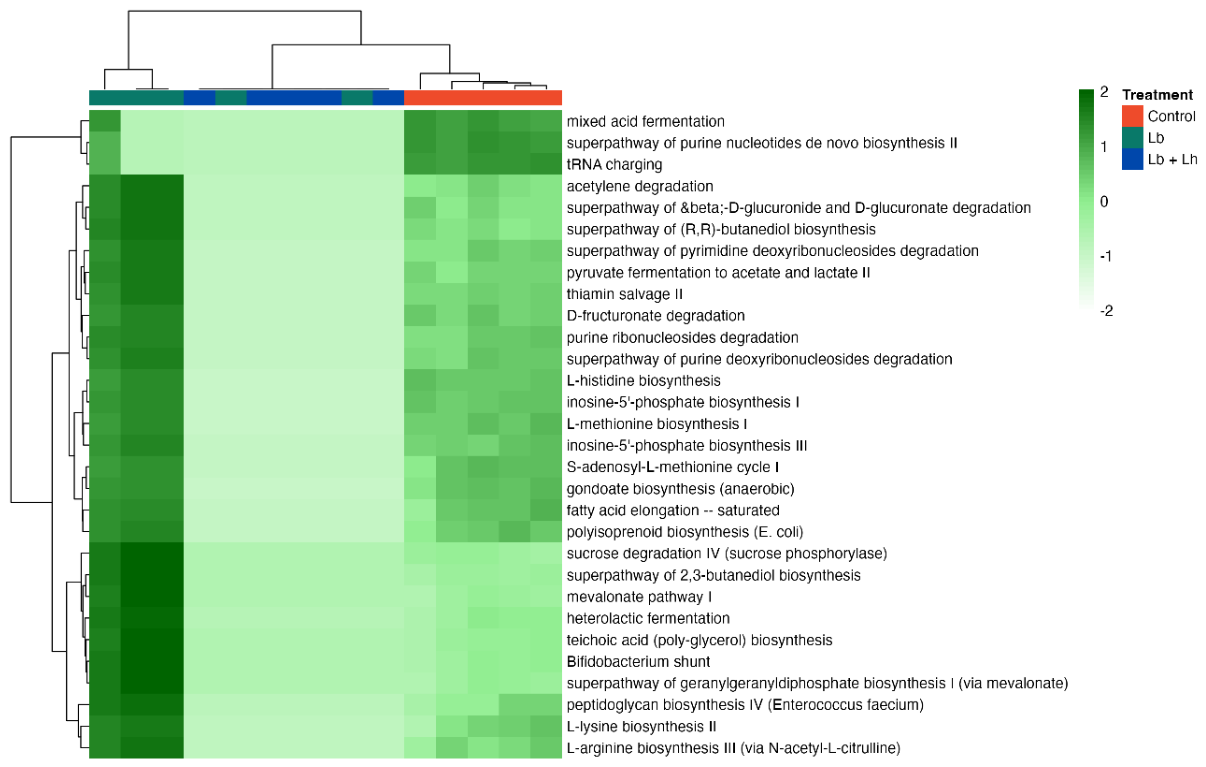
Gene prediction analysis revealed intense amino acid biosynthesis (e.g., L-ornithine biosynthesis, L-lysine biosynthesis VI, superpathway of L-threonine biosynthesis, superpathway of S-adenosyl-L-methionine biosynthesis) and carbohydrate degradation (e.g., mixed acid fermentation, D-fructuronate degradation, sucrose degradation IV via sucrose phosphorylase, superpathway of β-D-glucuronide and D-glucuronate degradation) at D20 in the inoculated groups compared to the control (Figure A11). This pattern shifted entirely at D60, where the control group exhibited significantly increased protein biosynthesis (Figure A12). At D100, a resurgence of anaerobic activity (e.g., heterolactic fermentation, pyruvate fermentation to acetate and lactate II, acetylene degradation) was observed in the inoculated groups compared to the control (Figure A13).
There was no significant direct correlation between the pH and temperature values with the LAB for any group.
4. Discussion
The pH remained low throughout the fermentation. Although values below 3.8 may raise concerns regarding the potential inhibition of LAB, no adverse effects were observed. In contrast, inoculated silages showed high LAB counts by D20, indicating that microbial activity was not impaired. The rapid consumption of WSCs and LA production contributed to the reduction in the pH, as well as the BA and NH3-N concentrations. The microbial succession took place right at D20, but with distinct patterns with Lentilactobacillus, as a major taxon in the inoculated silages, but moreso in the Lb + Lh, as this genus was more abundant compared to other indigenous LAB, such as Lactiplantibacillus, Lacticaseibacillus, and Secundilactobacillus. Xu et al. [33] reported similar results in sorghum silage inoculated with a L. buchneri strain combination, observing Lentilactobacillus dominance as early as three weeks post-inoculation. Lactiplantibacillus dominates native sorghum fermentation but shifts to Lentilactobacillus if inoculated, accelerating late-stage fermentation and highlighting its affinity for sorghum silage [33,34]. Lentilactobacillus has been associated with greater starch utilization efficiency during sorghum ensiling, fermenting protein–starch granules via proteolytic enzymes and with an optimal LA:AA ratio, which enhances silage fermentation and aerobic stability [2]. Though 16S rRNA-based microbial analysis is limited to genus-level resolution, the early post-inoculation effect may have been associated with L. hilgardii proliferation and the initial AA production, while L. buchneri later converted LA into AA and 1,2-propanediol [35,36]. The early metabolic activity of L. hilgardii, combined with the prolonged activity of L. buchneri, may have contributed to inhibition of spoilage-associated bacteria during silo opening in both the short and long term, a feature particularly relevant in semi-arid regions, where early silo opening is common due to forage scarcity [11,37]. At D60, the microbial succession ended with Lentilactobacillus as the dominant taxon, and there was no difference between the Lb and Lb + Lh, reflecting the transition to the fermentative equilibrium phase, as the availability of fermentable sugars decreased because, at this point, fermentation completely shifted from homolactic to heterofermentative, increasing the AA and PA concentrations observed at D60 and D100. The authors of [2,3] emphasized L. buchneri’s role in stabilizing silages by D45–D60, when AA levels curb spoilage, aligning with the authors of [4,9,38], who linked heterofermentative strains to higher aerobic stability via increased AA and microbial suppression.
In contrast, the microbial succession was undesirable at D60, suggesting that a greater relative abundance of non-LAB taxa made up most of the microbial composition. Paenibacillus and Acinetobacter are organic, acid-consuming bacteria linked to pH increases in silages, whereas Clostridium and Lelliottia can cause undesirable proteolysis, leading to biogenic amine formation, reducing the bioavailable protein content and inducing NH3+ formation, thereby lowering the overall fermented product quality [39,40]. Conversely, the NH3-N values remained below 100 g/kg of the total nitrogen, and even though the inoculated silages exhibited slightly higher NH3-N levels compared to the control, these values still reflected controlled protein fermentation [3,41,42]. This trend may be associated with the action of heterofermentative LAB, whose metabolic activity can contribute to ammonia release, even with the inhibition of enterobacteria by inoculants [43]. At D100, higher NH3-N in the Lb indicated CP degradation, while the Lb + Lh preserved protein better, highlighting the complementary roles of both inoculants at different stages of fermentation rather than a consistent synergistic effect across the entire ensiling process. The authors of [11] also observed low BA production in sorghum silages treated with L. buchneri and the combo, demonstrating these inoculants’ efficiency in preserving protein. This instability influenced DM losses during the aerobic phase, reflecting sorghum silage’s fermentative traits, where high WSCs and a low buffering capacity drive rapid acidification but increase susceptibility to deterioration and reduced aerobic stability. The acidification is faster when sorghum has high DM (≤33%), possibly creating an excessive amount of residual WSCs bound to plant proteins that could serve as a substrate for spoilage-associated microbes, and causing non-inoculated silage to show signs of deterioration even before exposure to air [8,33,44,45,46]. This may have favored the microbial succession at D60 toward the growth of non-LAB such as Paenibacillus, Acinetobacter, Clostridium, and Lelliottia in the control group. In this regard, both the Lb and Lb + Lh demonstrated greater efficiency in WSCs utilization, aiding silage preservation, while maintaining stable LA levels and lower WSCs variation during air exposure, which underscores the competitive superiority of heterofermentative inoculants over spoilage microorganisms, an effect particularly relevant in semi-arid regions, where the combination of high temperatures and low humidity can accelerate aerobic deterioration [34].
The residual WSCs may be offset by increased antifungal activity in L. buchneri-treated silages, where the acidified environment coupled with PA’s and AA’s antimicrobial activity enhance protection during storage and air exposure [21,38]. The Lb + Lh combination showed a tendency to enhance AA and AP production at specific time points, suggesting a potential additive or complementary effect on heterofermentative metabolism [4,8,10].
DM losses were controlled in the inoculated factorial treatments, with lower losses in the Lb at D20 and D60 due to AA’s inhibitory action on undesirable microbes, but at D100, AA and PA accumulation increased losses via compound volatilization [11,47]. Although heterofermentative LAB produce ethanol and CO2, which generate higher potential for DM losses, this does not equate to the ethanol-producing yeasts, which may explain inconsistent effects on DM recovery [4,48,49]. This is also corroborated by the observed OM reduction, which was probably caused by the heterofermentative metabolism of Lentilactobacillus over WSCs consumption [35,47]. The early-stage silage DM levels were similar across factorial treatments due to limited AA production and spoilage control, but by D60, the intensified heterofermentation in the Lb + Lh factorial treatments boosted AA and secondary metabolites, improving preservation yet increasing DM losses, while by D100, microbial metabolism balanced fermentative metabolites and DM retention. These results support [4,11] in highlighting heterofermentation regulation for optimal DM preservation, as inoculation reduced the LA:AA ratio in the Lb and Lb + Lh, increased AA production, and inhibited spoilage microorganisms, aligning with the authors of [50], who linked lower LA:AA ratios in sorghum silages to L. buchneri’s heterofermentative metabolism.
The absence of spoilage-associated microbes like Pichia, Candida, and Saccharomyces suggests that the high AA and anaerobic conditions acted as selective factors, while some yeasts, like Kazachstania, tolerated LA and may have contributed to early aerobic deterioration in low-pH silage, even with heterofermentative inoculants. This has been observed in different silages, including whole-plant corn, barley, and sugarcane tops [13,39,51]. Indeed, Kazachstania strains can grow and tolerate high osmolarity, acidity, and the presence of organic acids, ethanol, and salt, but the presence of yeasts does not necessarily indicate silage deterioration, as shown by the early presence of Kazachstania at D20, while the inoculated silages, particularly those treated with the L. buchneri and L. hilgardii combination, exhibited improved aerobic stability [52]. According to [8], the combination of L. buchneri and L. hilgardii in sorghum silage improves the fermentation quality and aerobic stability 15 days post-ensiling, highlighting these species’ adaptability to sorghum substrates. The absence of yeasts at D100 was likely due to the acidic silage pH (3.28–3.37), which created an unfavorable environment for fungal growth, supporting the studies [53,54] on the antifungal role of low pH. The increased AA and PA concentrations in treated silages hampered fungal growth and delayed aerobic deterioration. The lower LA:AA ratio in treated silages reflects more efficient heterofermentative fermentation, stabilizing the profile against oxygen exposure, while the prolonged activity of Lentilactobacillus from D60 onward enhances antimicrobial metabolite production, controlling fungal growth and improving the aerobic stability. The use of heterofermentative strains minimizes the high-temperature exposure and prevents spoilage microbes upon oxygen contact owing to AA’s role in inhibiting yeasts and mols, thereby improving the aerobic stability in L. buchneri-treated sorghum silages [11,38,55]. Notwithstanding, the Lb + Lh showed advantages in specific variables and time points, particularly related to fungal inhibition from D60 onward, although these effects were not consistently superior to Lb alone across all evaluated parameters. Organic acids can effectively inhibit fungi in heterofermentative-inoculated sorghum silages [8,10]. We acknowledge that qPCR should have been included to quantify the absolute bacterial abundance in the silage, as our results reflect the community composition rather than the total bacterial load, limiting links to metabolic activity, such as mycotoxin production and feed deterioration [56].
5. Conclusions
Inoculation with L. buchneri, either alone or in combination with L. hilgardii, improved the preservation and aerobic stability of sorghum silage. Although the combined inoculant promoted more stable microbial succession at 100 days and greater early abundance of Lentilactobacillus (20 days), its efficacy did not consistently surpass that of the isolated application of L. buchneri across all evaluated fermentative and bromatological parameters.
Author Contributions
Writing—original draft, writing—review and editing, methodology, investigation, data curation: L.M.P.R. Supervision, data curation, formal analysis, software, validation, writing—review and editing: A.J.d.S.M. Supervision, resources, project administration, funding acquisition, conceptualization: E.M.S., D.d.J.F., J.S.d.O. and A.d.M.Z. Investigation, data curation: P.d.C.T.J., G.M.L., C.B.d.M.C., A.H.A. and G.R.d.M. Data curation, formal analysis, software, validation, writing—review and editing: M.L.P.L. and J.P.d.F.R. All authors have read and agreed to the published version of the manuscript.
Funding
This research was funded by the Paraíba State Research Foundation (FAPESQ) (2023/2396) grant.
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
The datasets generated during or analyzed during the current study are available from the corresponding author upon reasonable request.
Acknowledgments
The authors thank the Paraíba State Research Foundation (FAPESQ), the National Council for Scientific and Technological Development (CNPq), the Coordination for the Improvement of Higher Education Personnel (CAPES), Finance Code 001, the State Foundation for the Support of Research and Scientific and Technological Development (FAPEMA-Brazil) and the National Institute of Science and Technology in Animal Science (INCT-CA) for all their support and assistance.
Conflicts of Interest
The authors declare no conflicts of interest.
Abbreviations
The following abbreviations are used in this manuscript:
| AA | Acetic acid |
| BA | Butyric acid |
| BC | Buffering capacity |
| CFUs | Colony-forming units |
| CP | Crude protein |
| D20 | 20 days |
| D60 | 60 days |
| D100 | 100 days |
| DM | Dry matter |
| FM | Fresh matter |
| FP | Fermentation period |
| LA | Lactic acid |
| LAB | Lactic acid bacteria |
| Lb | Lentilactobacillus buchneri |
| Lh | Lentilactobacillus hilgardii |
| NDF | Neutral detergent fiber |
| NH3-N | Ammonia nitrogen |
| OM | Organic matter |
| PA | Propionic acid |
| WSCs | Water-soluble carbohydrates |
Appendix A
Figure A1.
Alpha bacterial diversity indices (observed, Shannon, Simpson, Pielou, and Faith’s PD) in sorghum silages inoculated with microbial additives during fermentation periods of 20, 60, and 100 days. D20: sorghum forage-based silage after 20 days of fermentation; D60: sorghum forage-based silage after 60 days of fermentation; D100: inoculated sorghum forage-based silage after 100 days of fermentation. Control: control (without inoculant); Lb: strain Lentilactobacillus buchneri; Lb + Lh: Lentilactobacillus hilgardii CNCM I 4785 combined with L. buchneri NCIMB 40788.
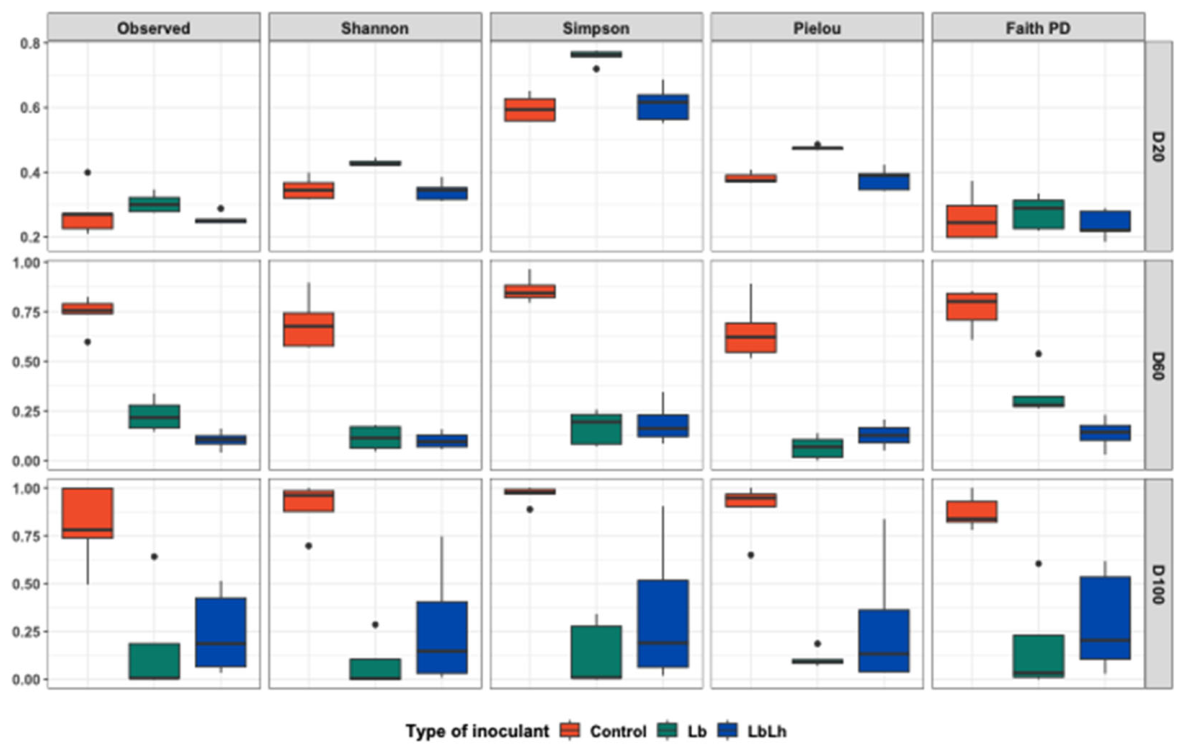
Figure A2.
Fungal alpha diversity indices (observed, Shannon, Simpson, Pielou, and Faith’s PD) in sorghum silages inoculated with microbial additives during fermentation periods of 20, 60, and 100 days. D20: sorghum forage-based silage after 20 days of fermentation; D60: sorghum forage-based silage after 60 days of fermentation; D100: inoculated sorghum forage-based silage after 100 days of fermentation. Control: control (without inoculant); Lb: strain Lentilactobacillus buchneri; Lb + Lh: Lentilactobacillus hilgardii CNCM I 4785 combined with L. buchneri NCIMB 40788.
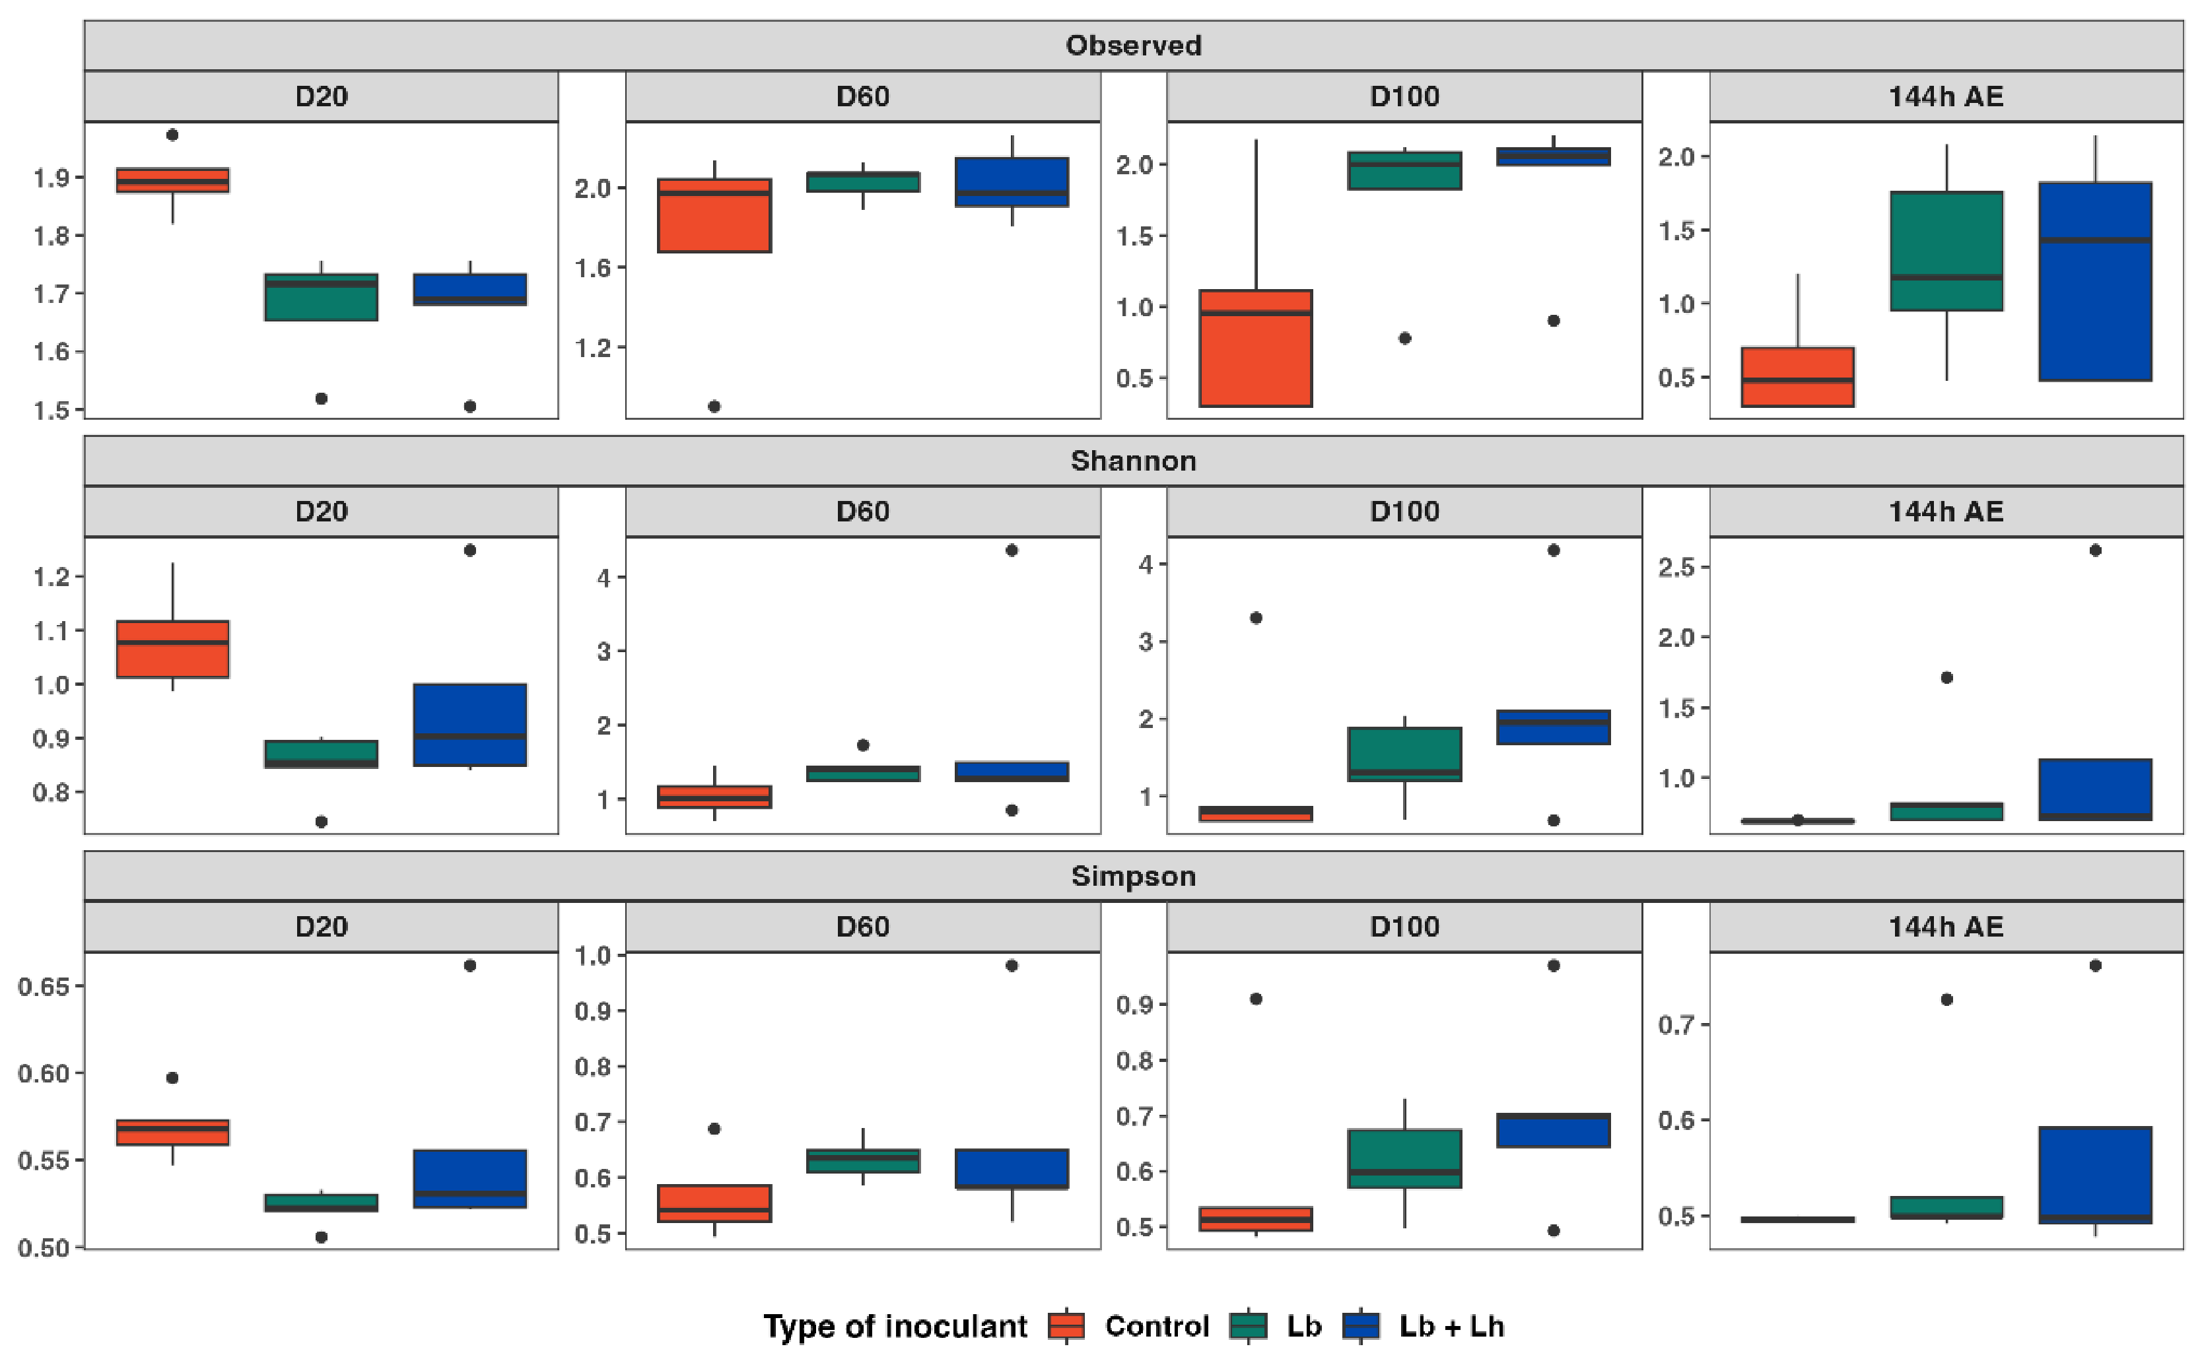
Figure A3.
Relative abundances of bacterial phyla in sorghum silages inoculated with microbial additives during fermentation periods of 20, 60, and 100 days. D20: sorghum forage-based silage after 20 days of fermentation; D60: sorghum forage-based silage after 60 days of fermentation; D100: inoculated sorghum forage-based silage after 100 days of fermentation. Control: control (without inoculant); Lb: strain Lentilactobacillus buchneri; Lb + Lh: Lentilactobacillus hilgardii CNCM I 4785 combined with L. buchneri NCIMB 40788.
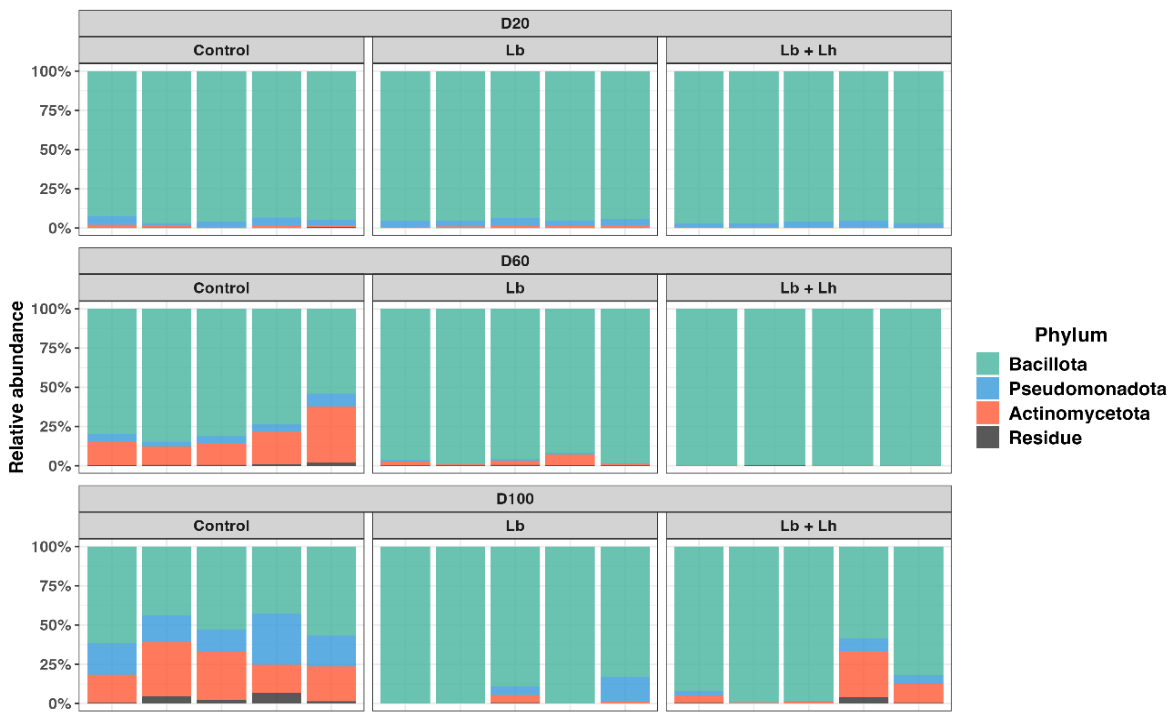
Figure A4.
Relative abundances of fungal phyla in sorghum silages inoculated with microbial additives during fermentation periods of 20, 60, and 100 days and after 144 h of aerobic exposure. D20: sorghum forage-based silage after 20 days of fermentation; D60: sorghum forage-based silage after 60 days of fermentation; D100: inoculated sorghum forage-based silage after 100 days of fermentation; 144 h. AE: silage exposed to air for 144 h. Control: control (without inoculant); Lb: strain Lentilactobacillus buchneri; Lb + Lh: Lentilactobacillus hilgardii CNCM I 4785 combined with L. buchneri NCIMB 40788.
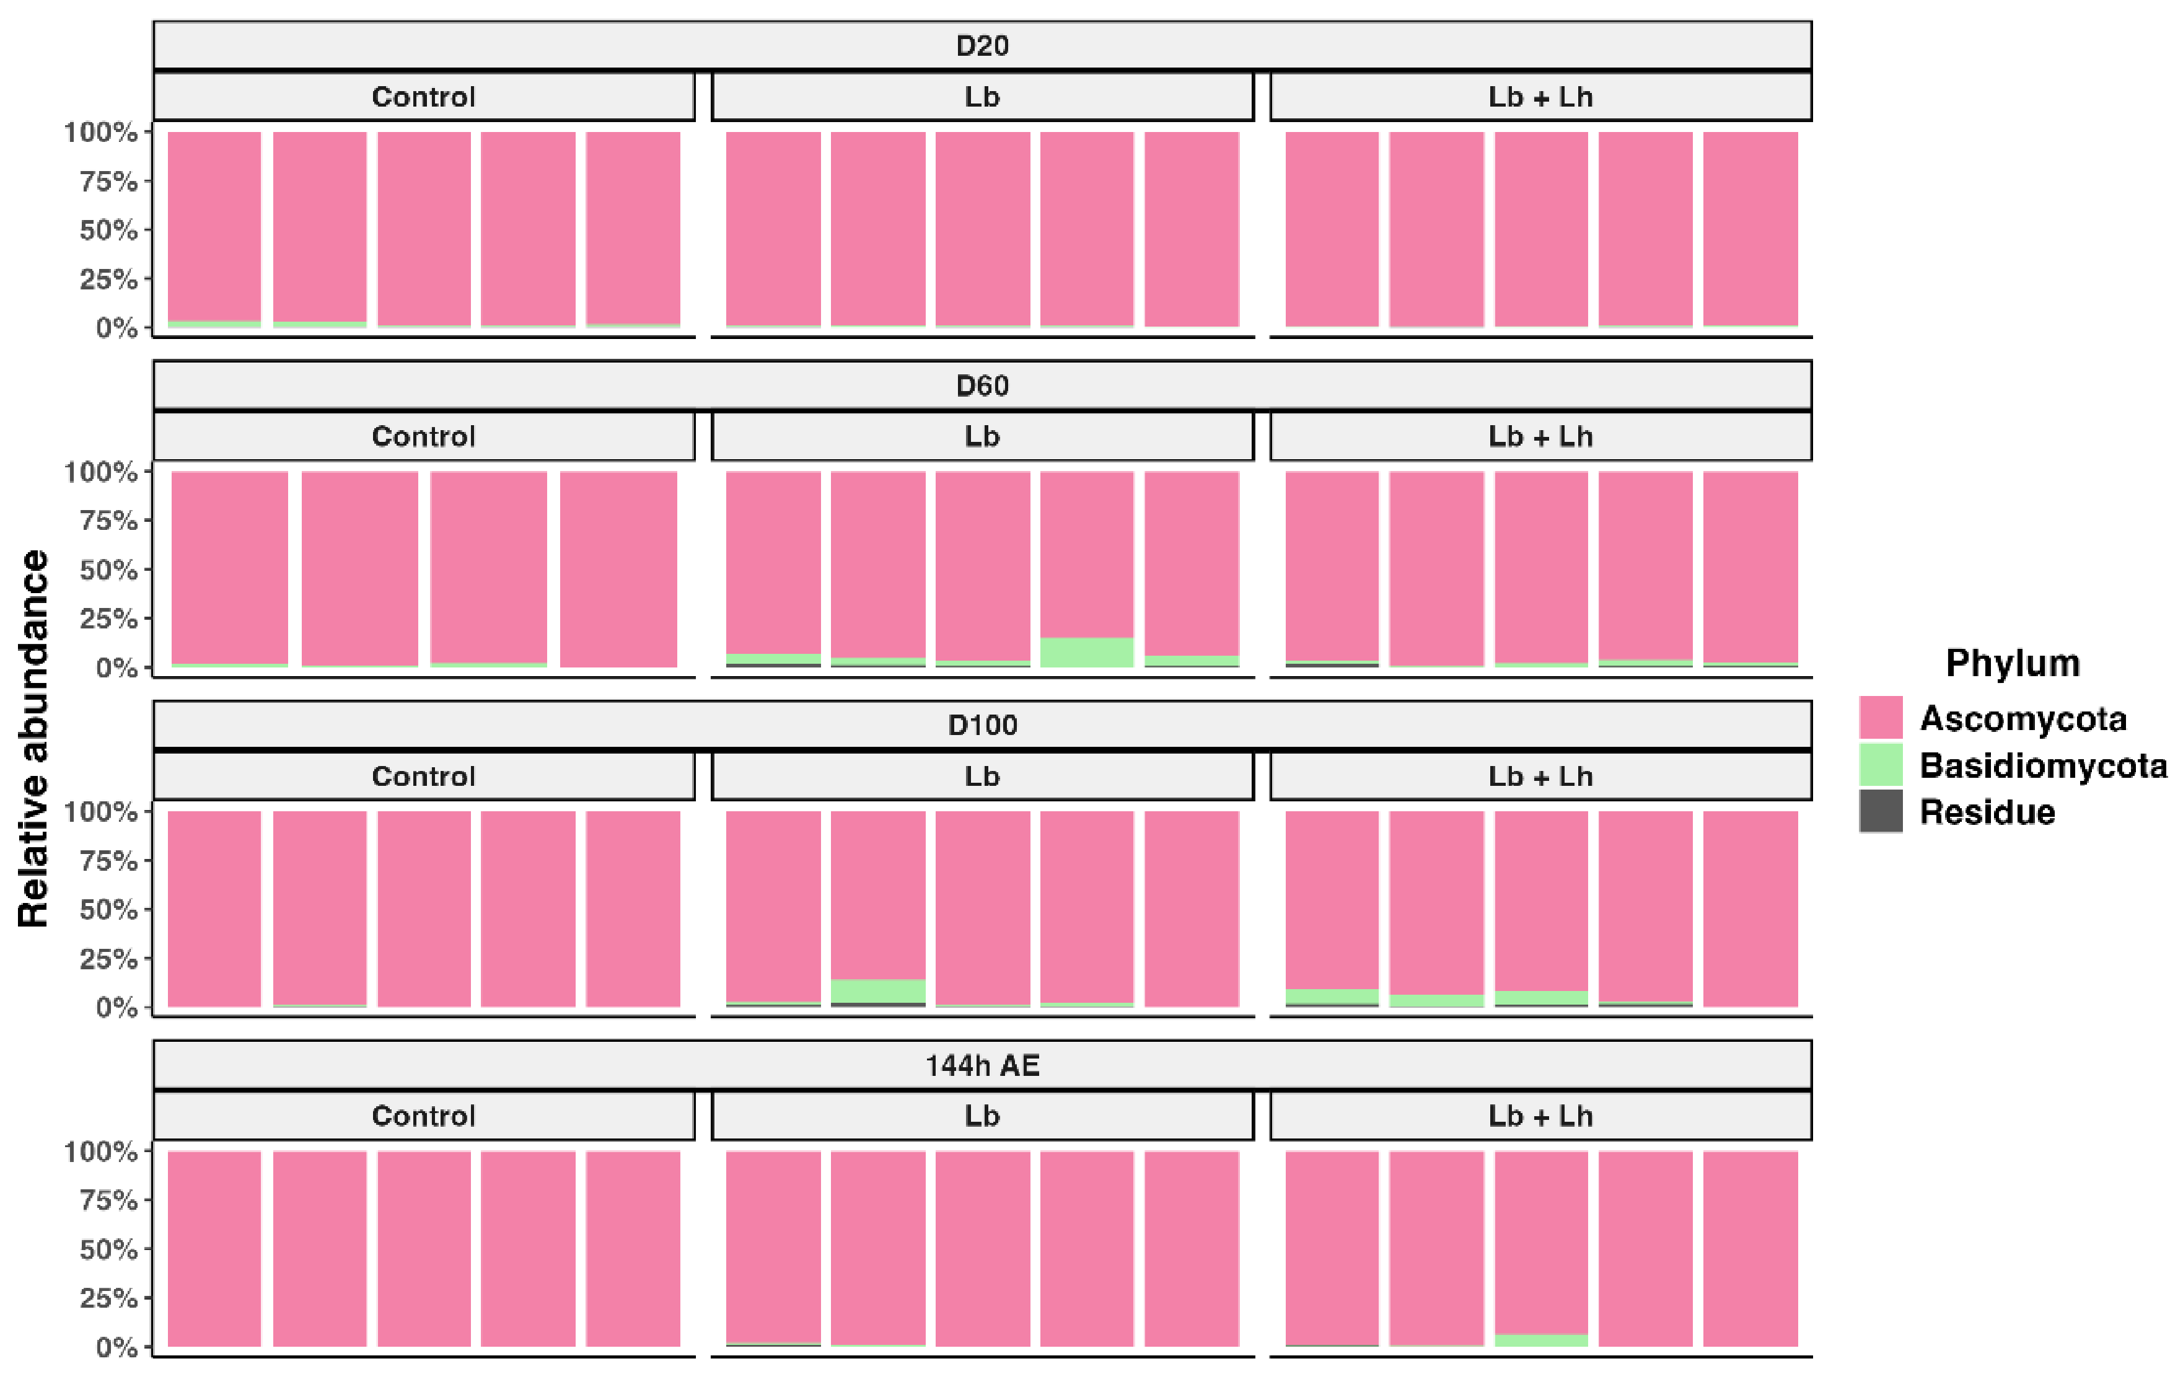
Figure A5.
Relative abundances of bacterial families in sorghum silages inoculated with microbial additives during fermentation periods of 20, 60, and 100 days. D20: sorghum forage-based silage after 20 days of fermentation; D60: sorghum forage-based silage after 60 days of fermentation; D100: inoculated sorghum forage-based silage after 100 days of fermentation. Control: control (without inoculant); Lb: strain Lentilactobacillus buchneri; Lb + Lh: Lentilactobacillus hilgardii CNCM I 4785 combined with L. buchneri NCIMB 40788.
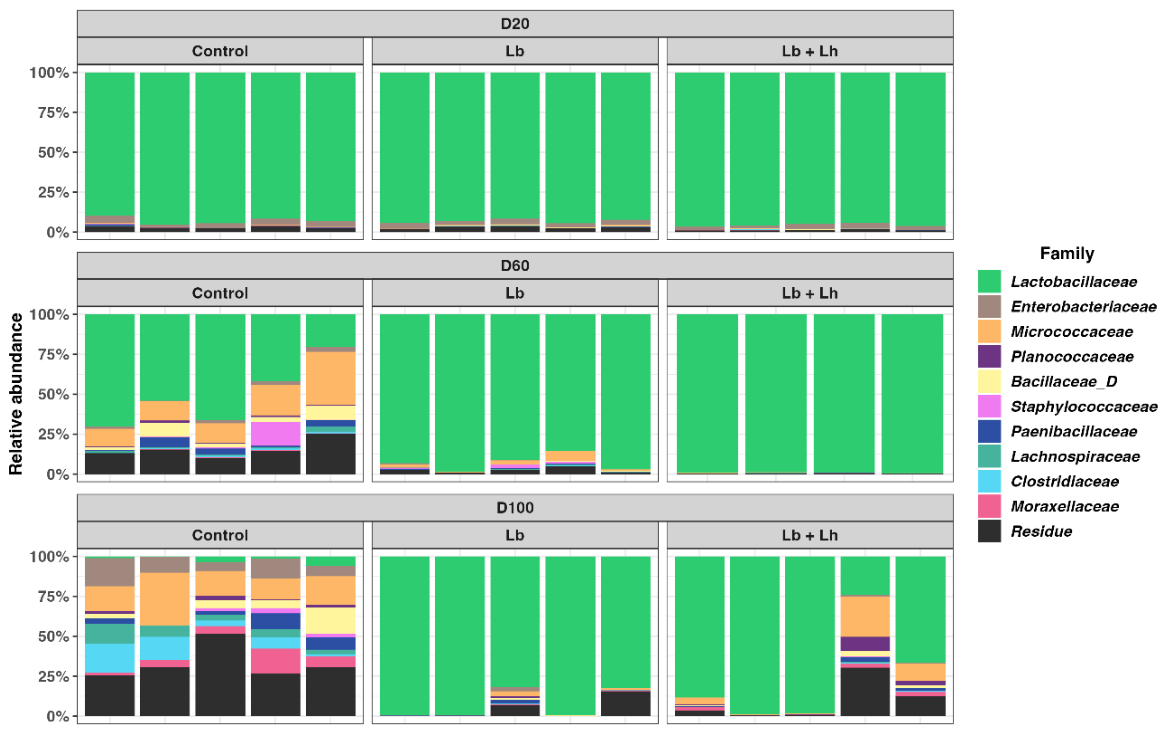
Figure A6.
Relative abundances of fungal families in sorghum silages inoculated with microbial additives during fermentation periods of 20, 60, and 100 days and after 144 h of aerobic exposure. D20: sorghum forage-based silage after 20 days of fermentation; D60: sorghum forage-based silage after 60 days of fermentation; D100: inoculated sorghum forage-based silage after 100 days of fermentation; 144 h. AE: silage exposed to air for 144 h. Control: control (without inoculant); Lb: strain Lentilactobacillus buchneri; Lb + Lh: Lentilactobacillus hilgardii CNCM I 4785 combined with L. buchneri NCIMB 40788.
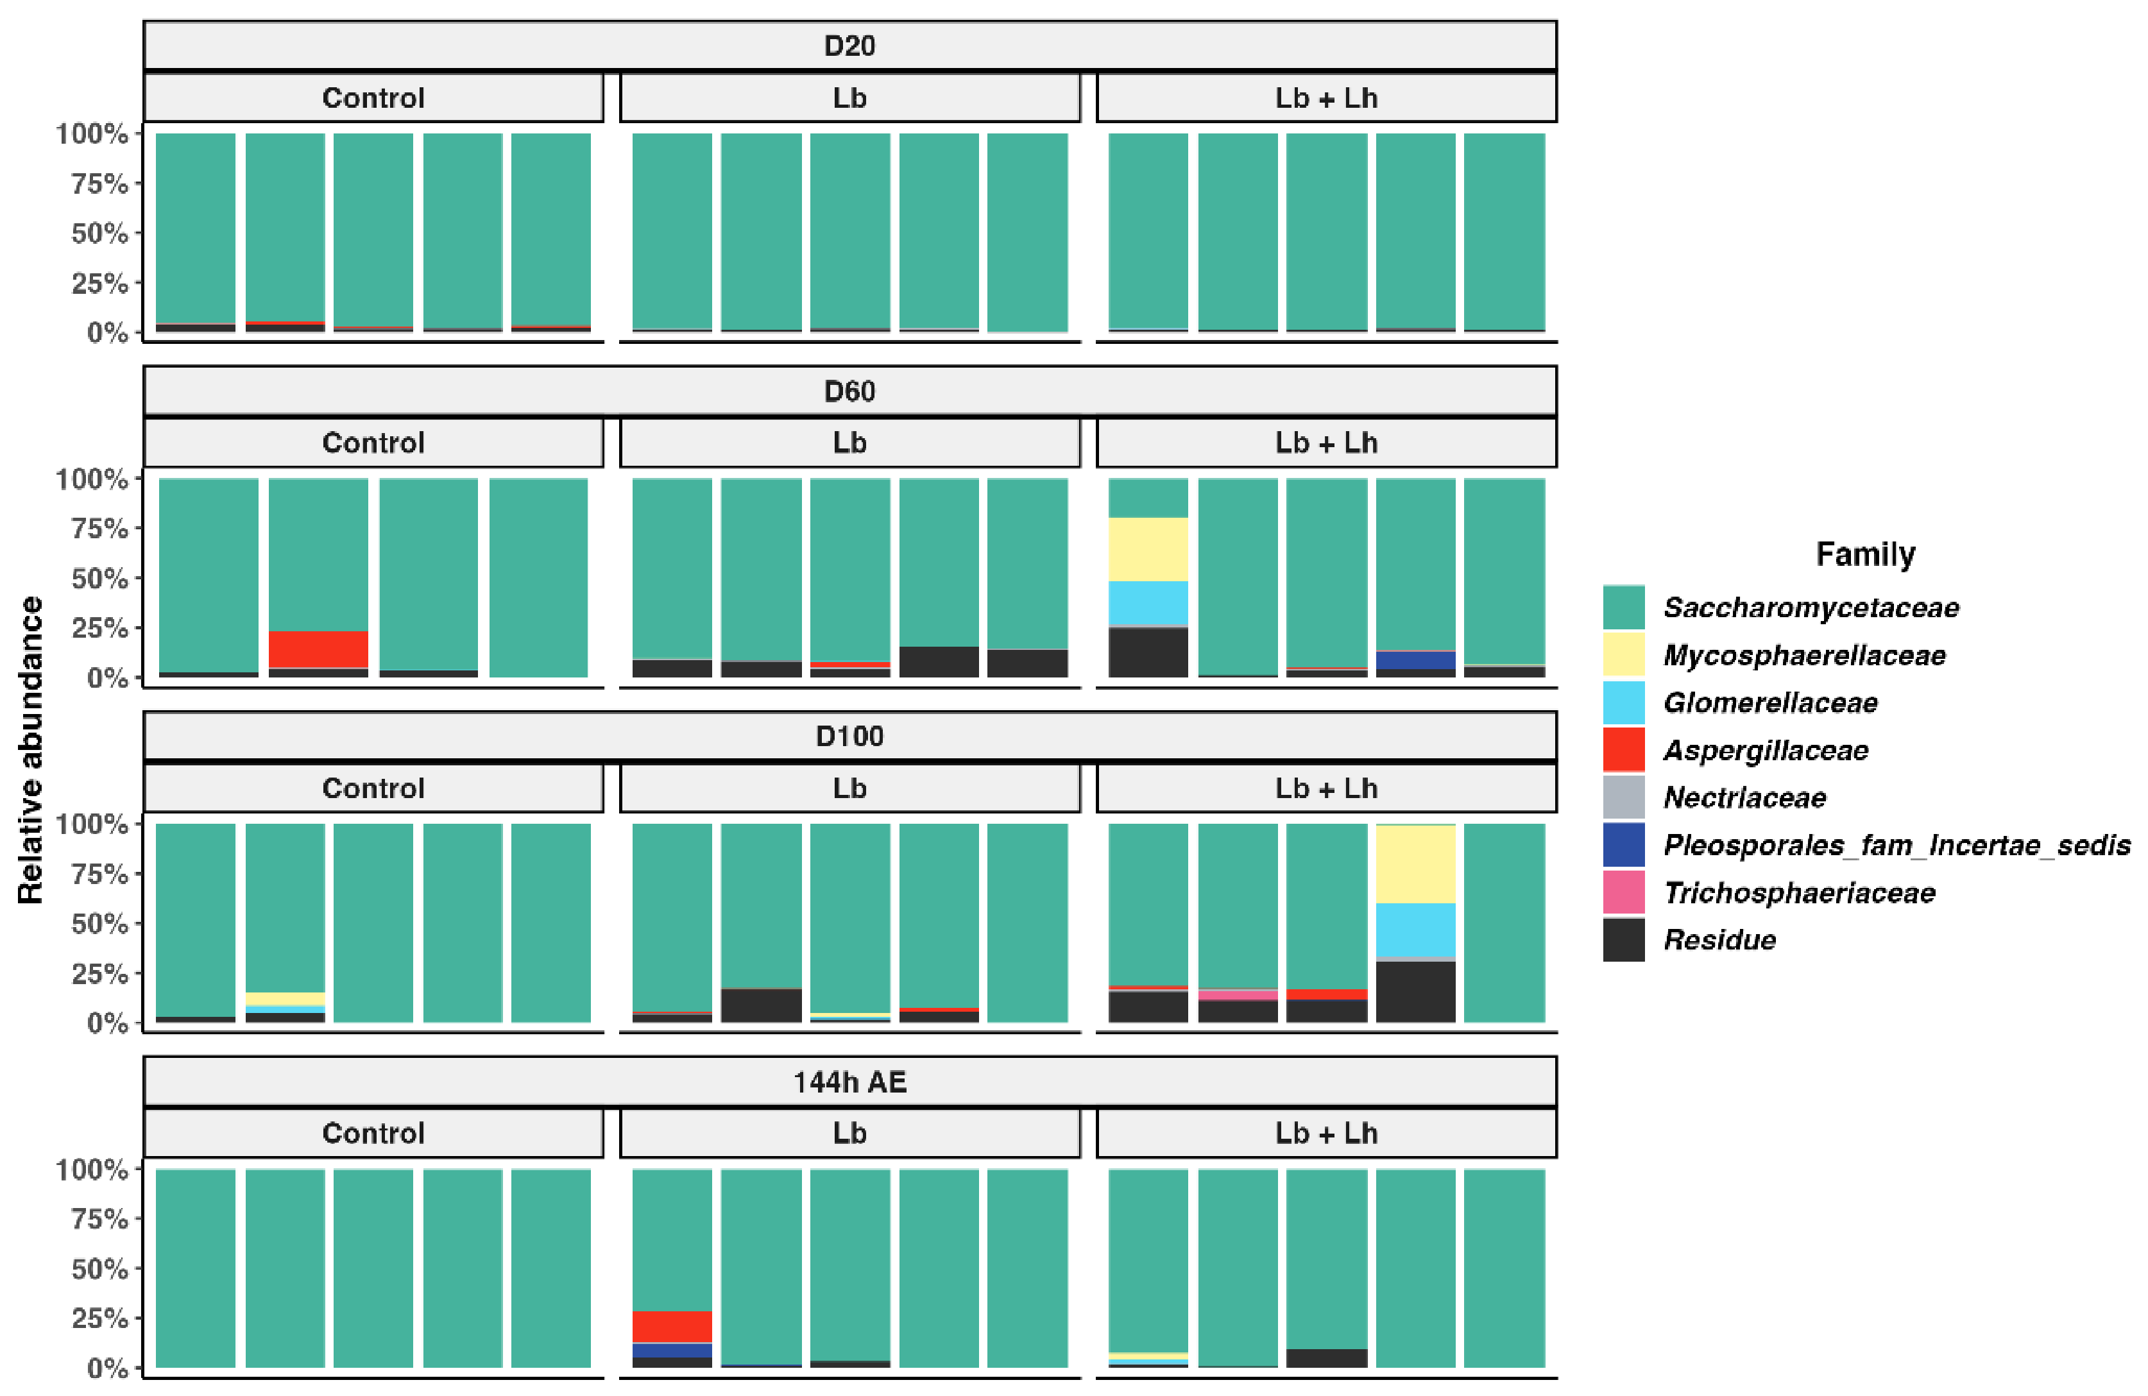
Figure A7.
Differential abundances of bacteria in sorghum silages inoculated with microbial additives after 20 days of fermentation. D20: sorghum forage-based silage after 20 days of fermentation. Control: control (without inoculant); Lb: strain Lentilactobacillus buchneri; Lb + Lh: Lentilactobacillus hilgardii CNCM I 4785 combined with L. buchneri NCIMB 40788.
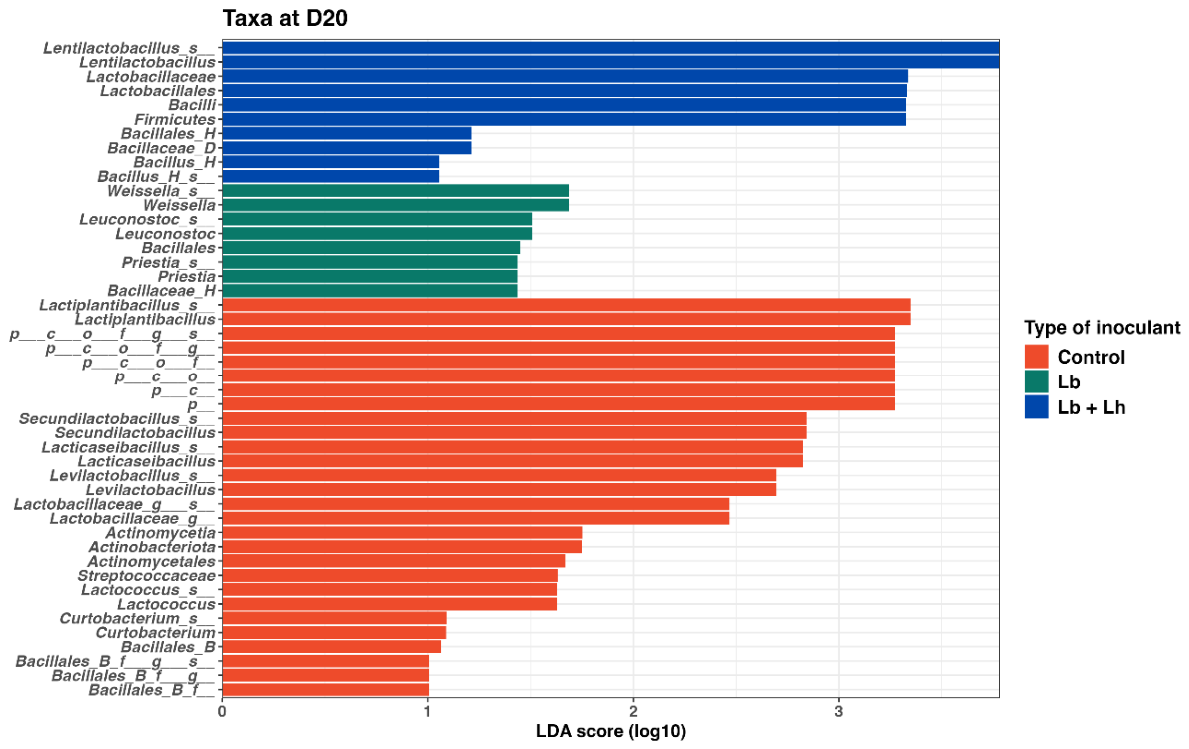
Figure A8.
Differential abundances of bacteria in sorghum silages inoculated with microbial additives after 60 days of fermentation. D60: sorghum forage-based silage after 60 days of fermentation. Control: control (without inoculant); Lb + Lh: Lentilactobacillus hilgardii CNCM I 4785 combined with L. buchneri NCIMB 40788.
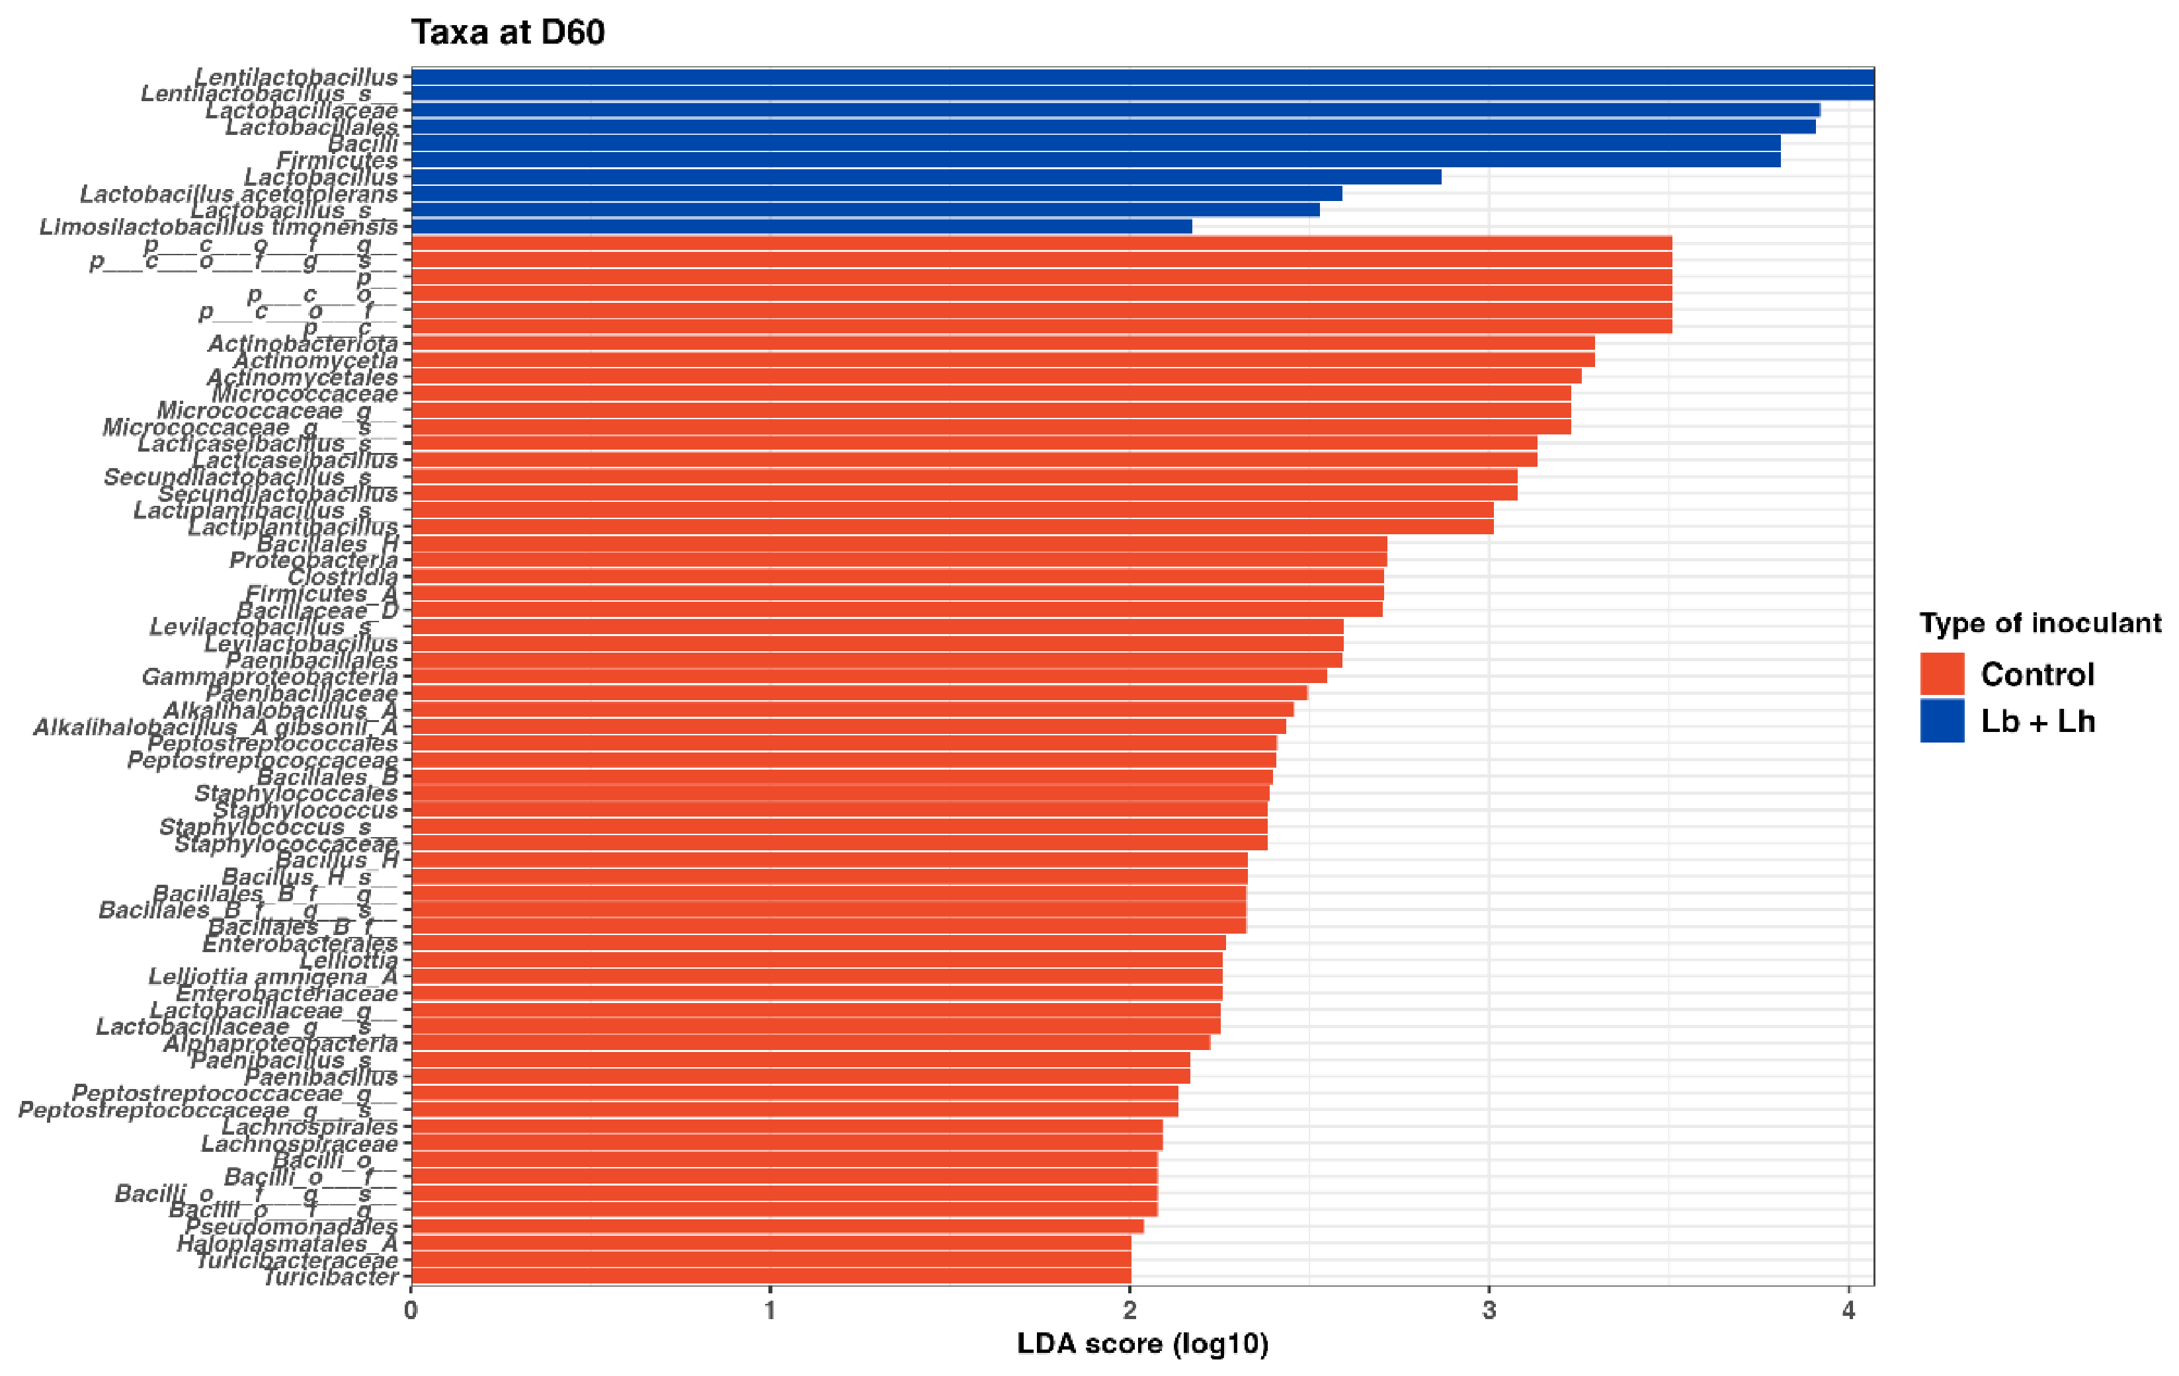
Figure A9.
Differential abundances of bacteria in sorghum silages inoculated with microbial additives after 100 days of fermentation. D100: inoculated sorghum forage-based silage after 100 days of fermentation. Control: control (without inoculant); Lb: strain Lentilactobacillus buchneri.
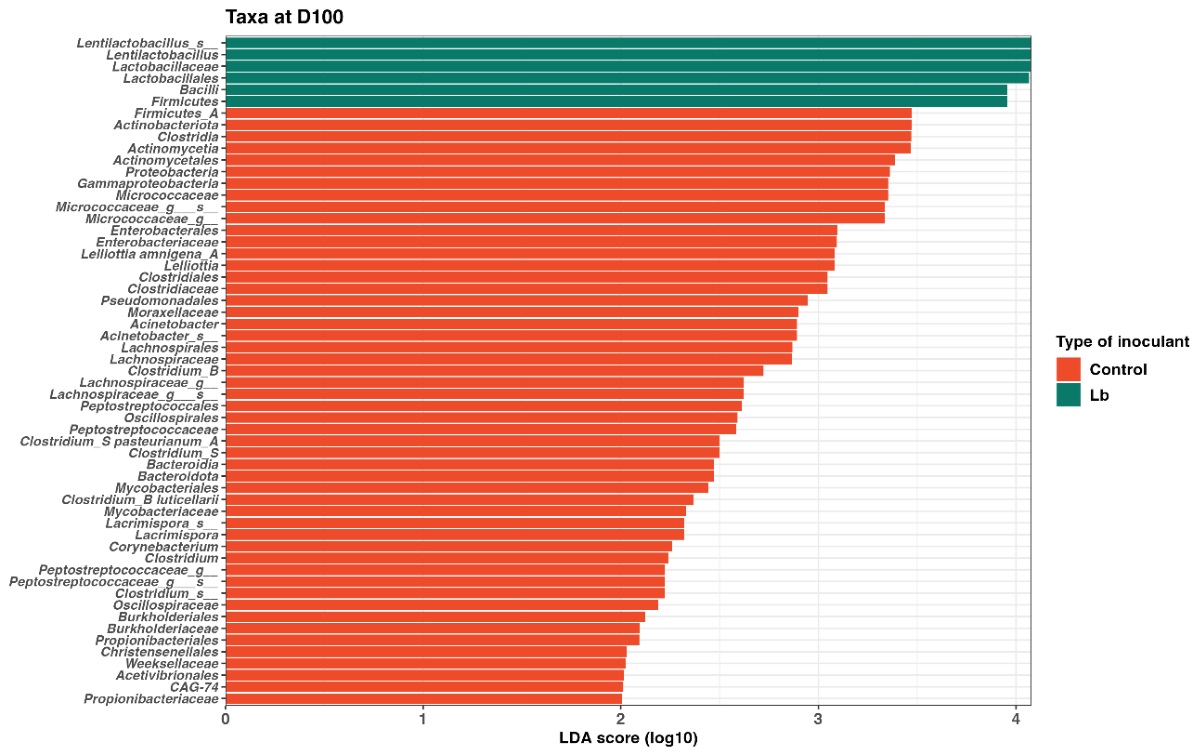
Figure A10.
Relative abundances of fungal genera in sorghum silages inoculated with microbial additives during fermentation periods of 20, 60, and 100 days and after 144 h of aerobic exposure. D20: sorghum forage-based silage after 20 days of fermentation; D60: sorghum forage-based silage after 60 days of fermentation; D100: inoculated sorghum forage-based silage after 100 days of fermentation; 144 h. AE: silage exposed to air for 144 h. Control: control (without inoculant); Lb: strain Lentilactobacillus buchneri; Lb + Lh: Lentilactobacillus hilgardii CNCM I 4785 combined with L. buchneri NCIMB 40788.
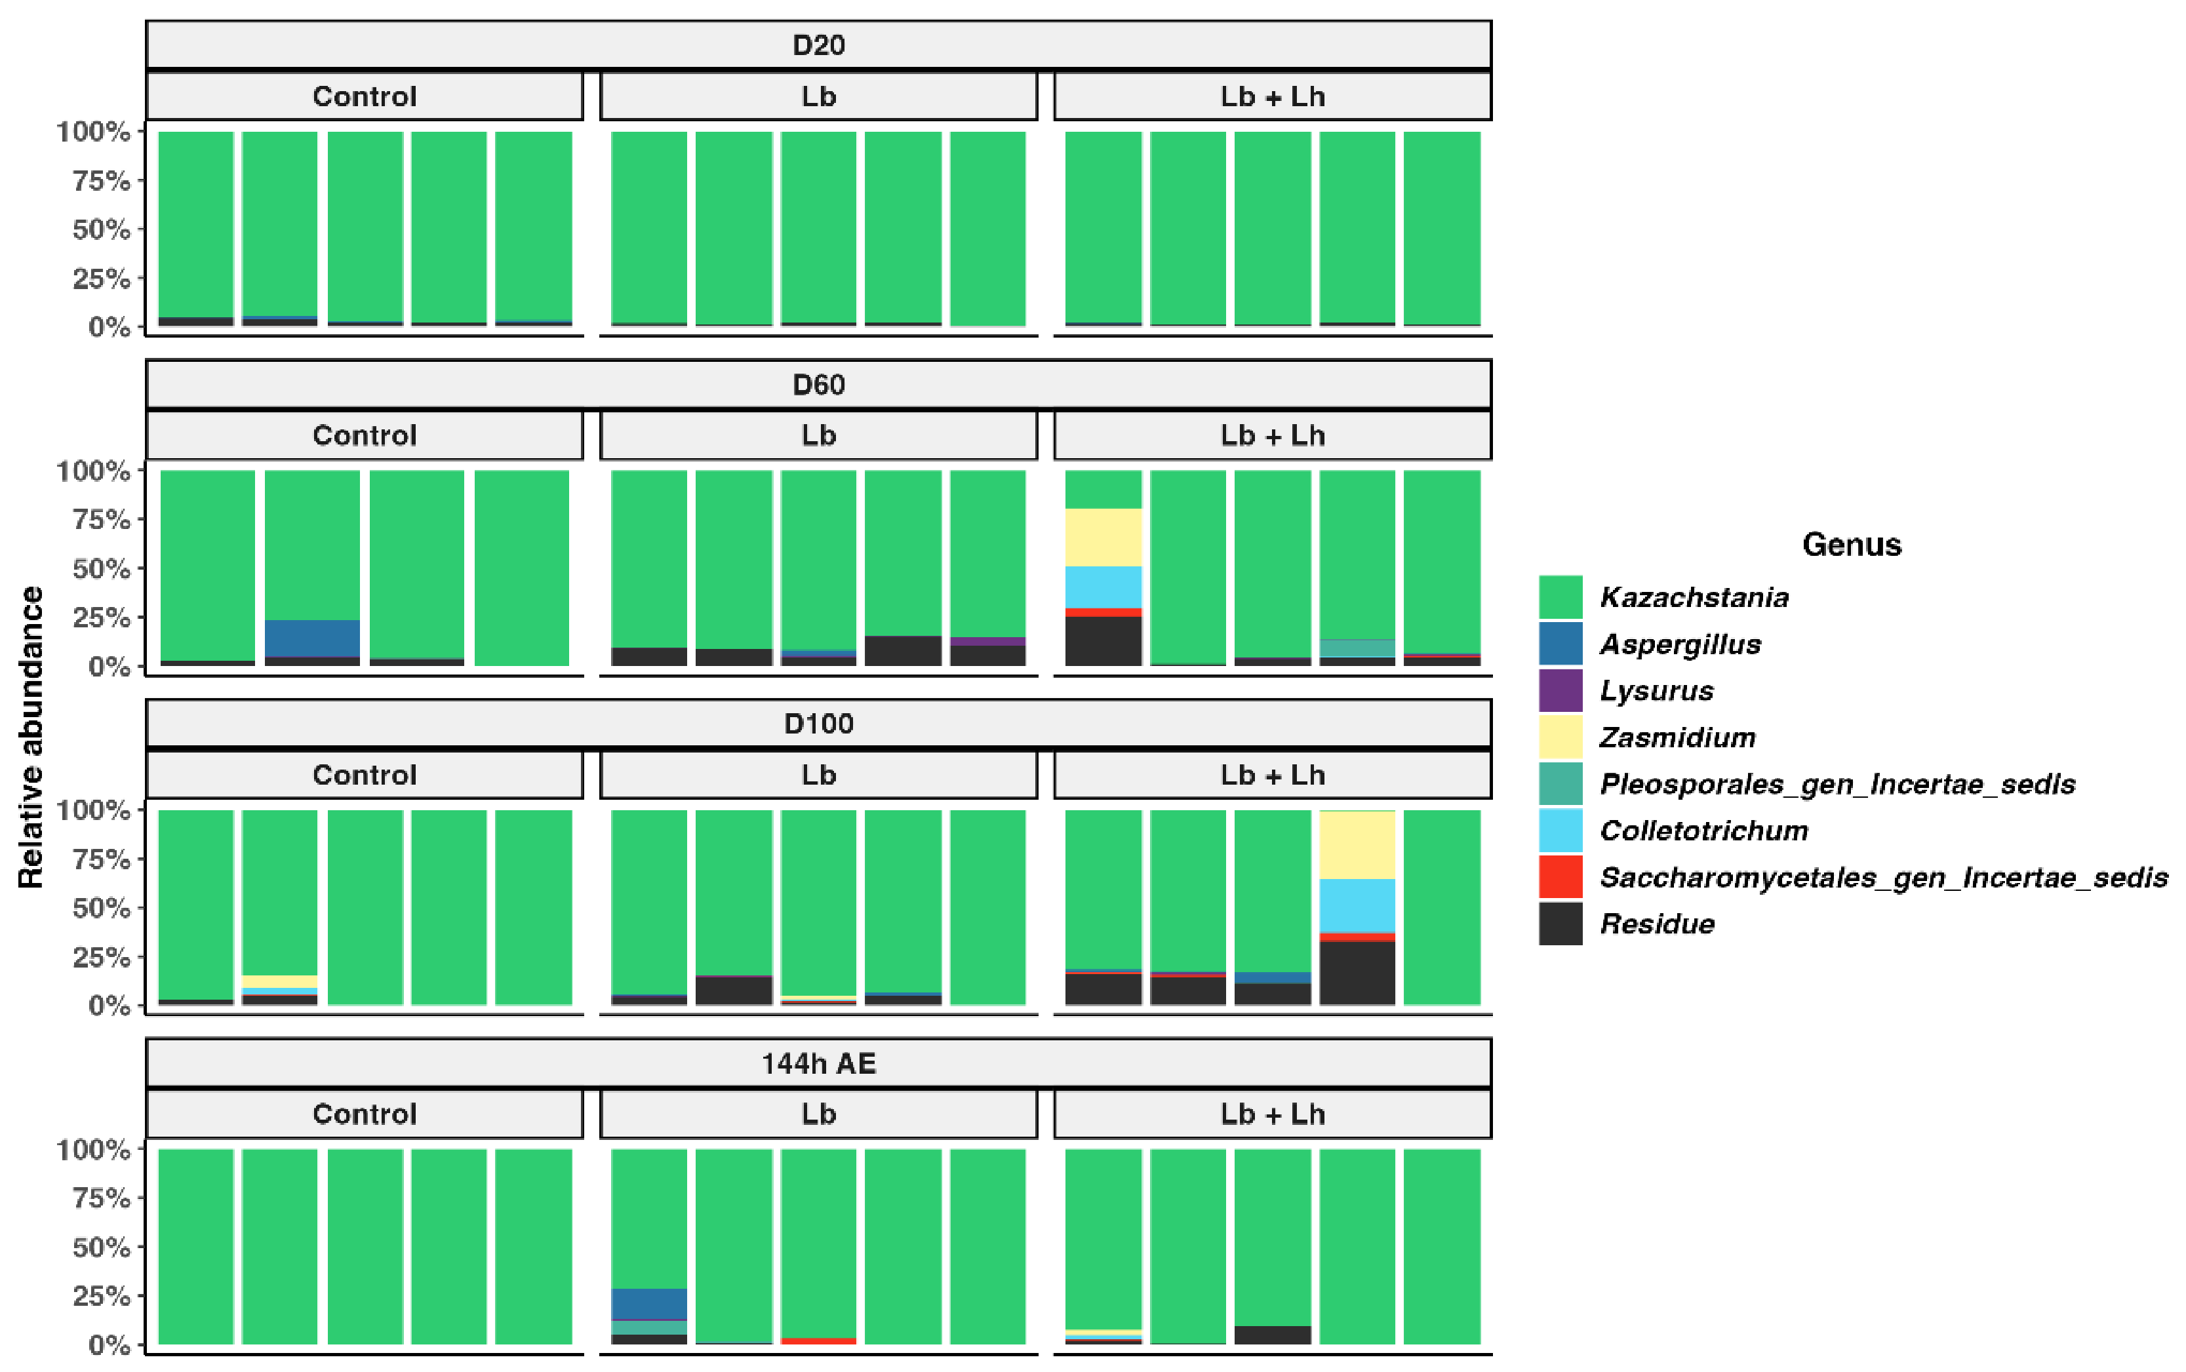
Figure A11.
Gene prediction of bacteria in sorghum silages inoculated with microbial additives after 20 days of fermentation. Control: control (without inoculant); Lb: strain Lentilactobacillus buchneri; Lb + Lh: Lentilactobacillus hilgardii CNCM I 4785 combined with L. buchneri NCIMB 40788.
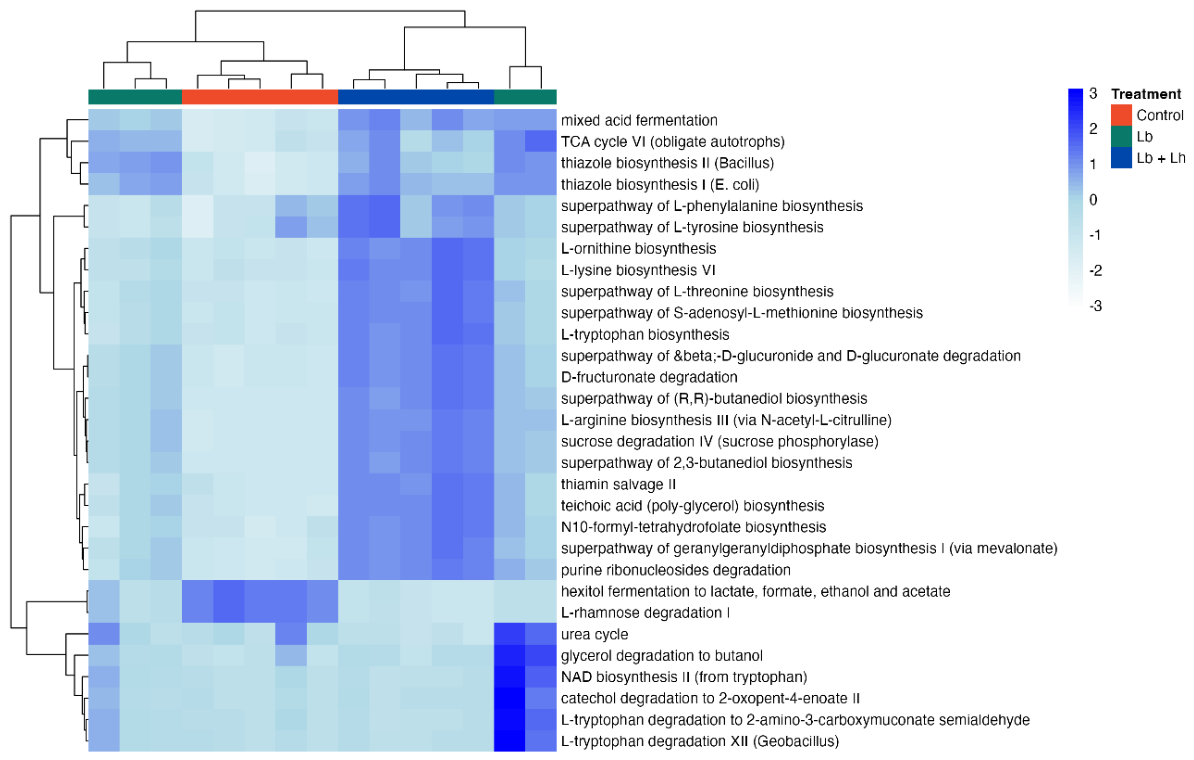
Figure A12.
Gene prediction of bacteria in sorghum silages inoculated with microbial additives after 60 days of fermentation. Control: control (without inoculant); Lb: strain Lentilactobacillus buchneri; Lb + Lh: Lentilactobacillus hilgardii CNCM I 4785 combined with L. buchneri NCIMB 40788.
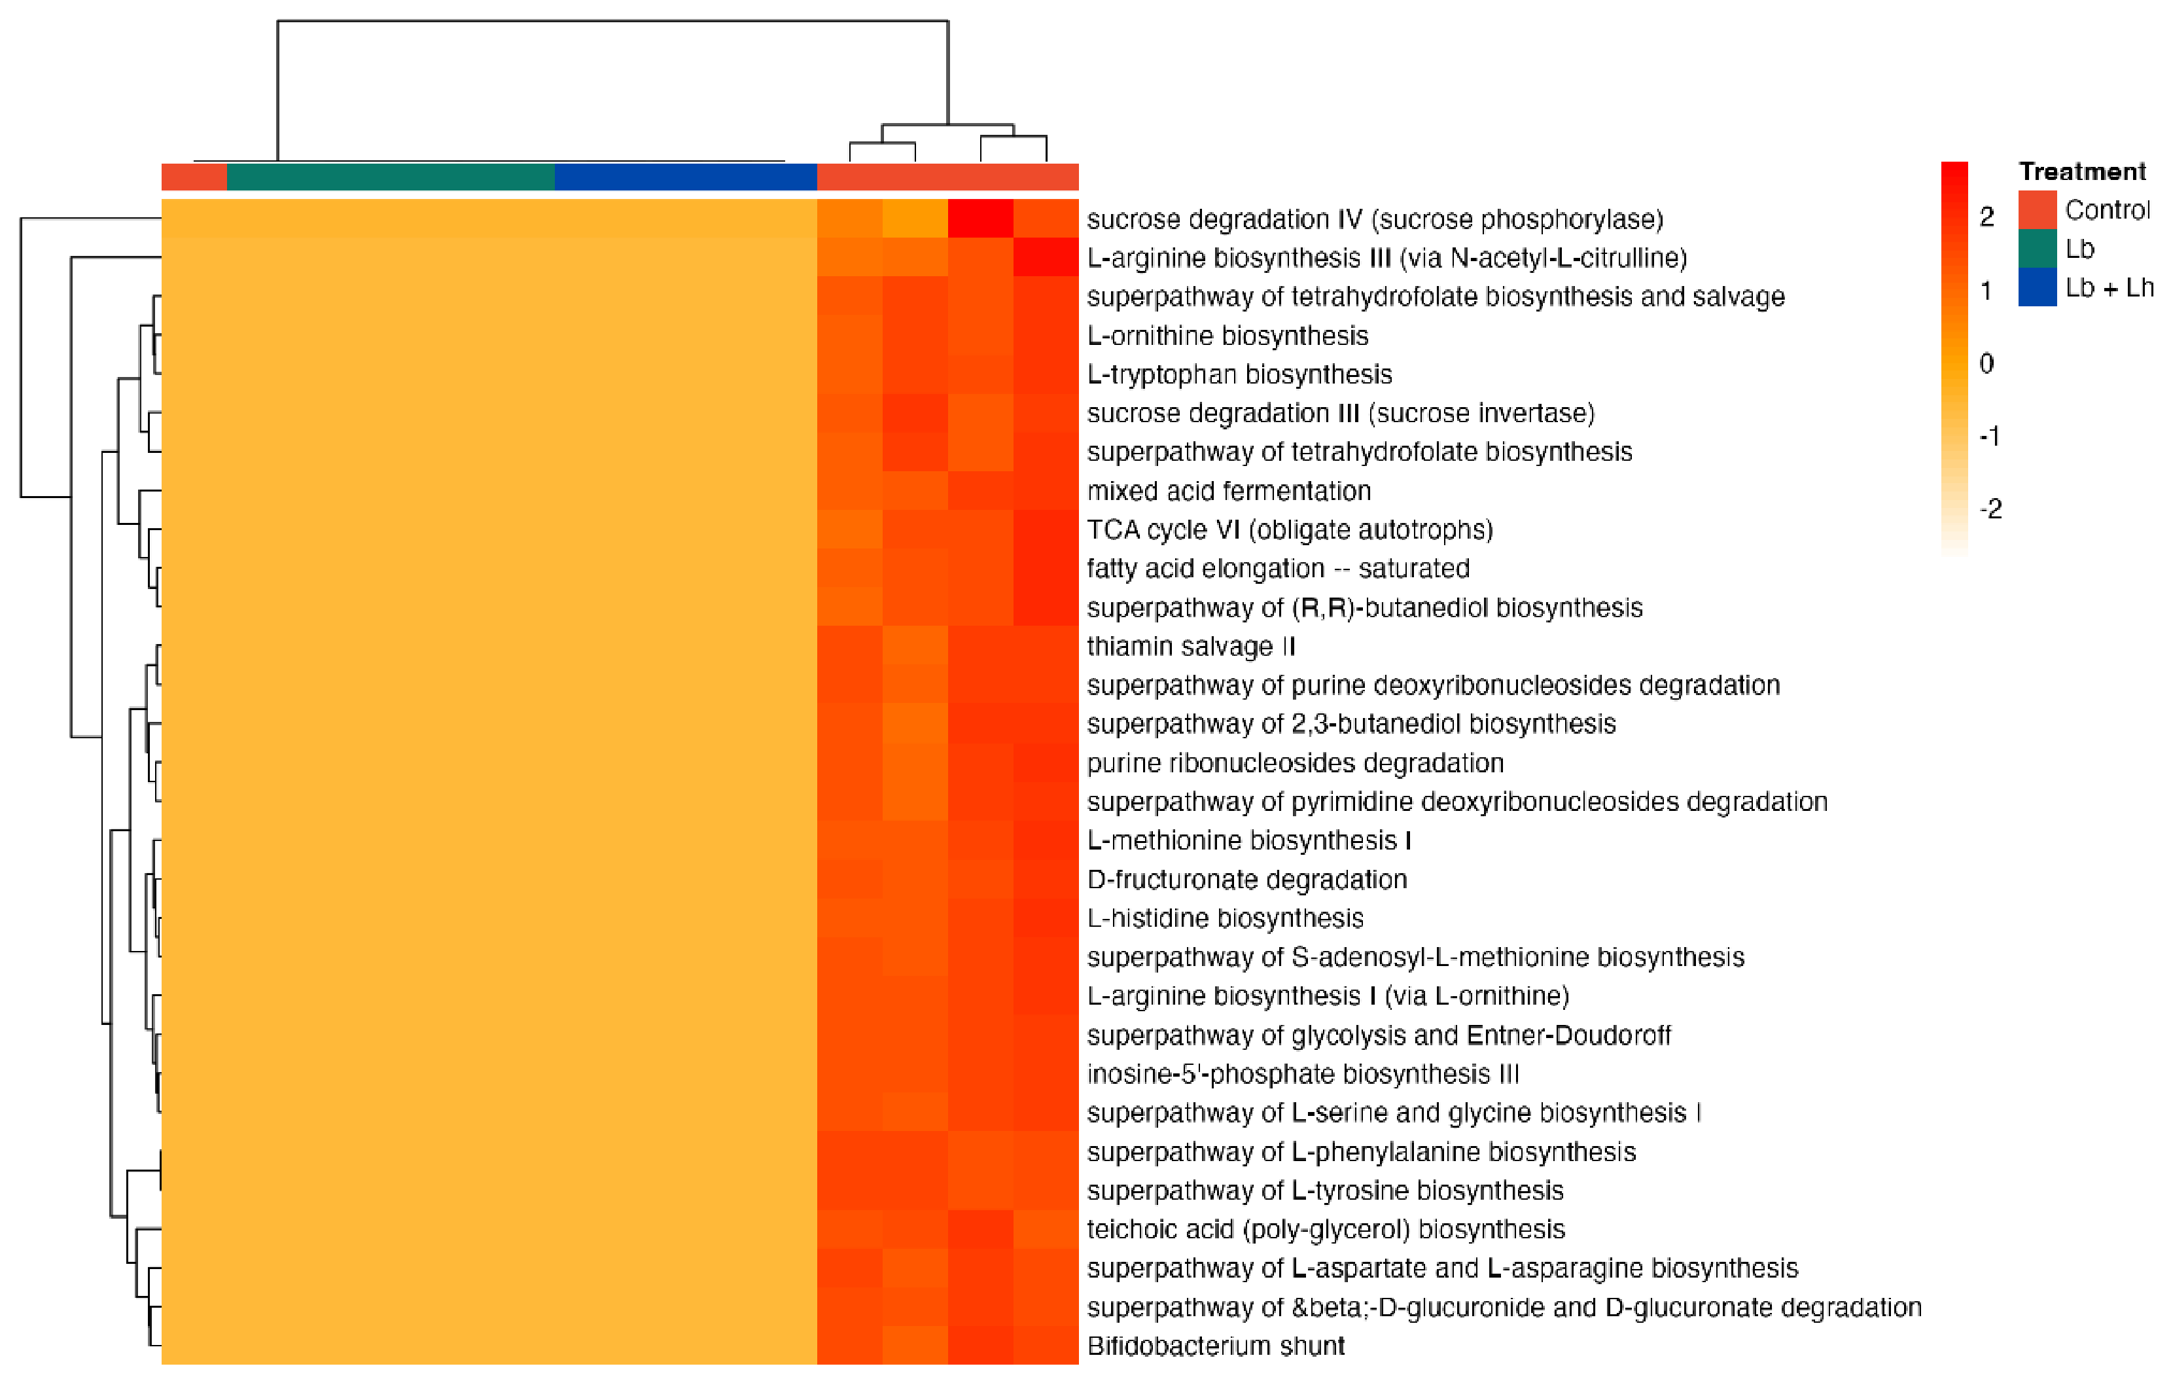
Figure A13.
Gene prediction of bacteria in sorghum silages inoculated with microbial additives after 100 days of fermentation. Control: control (without inoculant); Lb: strain Lentilactobacillus buchneri; Lb + Lh: Lentilactobacillus hilgardii CNCM I 4785 combined with L. buchneri NCIMB 40788.
References
- Khalifa, M.; Eltahir, E.A.B. Assessment of global sorghum production, tolerance, and climate risk. Front. Sustain. Food Syst. 2023, 7, 1184373. [Google Scholar] [CrossRef] [Scilit]
- Muck, R.E.; Nadeau, E.M.G.; McAllister, T.A.; Contreras-Govea, F.E.; Santos, M.C.; Kung, L. Silage review: Recent advances and future uses of silage additives. J. Dairy Sci. 2018, 101, 3980–4000. [Google Scholar] [CrossRef] [Scilit]
- Kung, L.; Shaver, R.D.; Grant, R.J.; Schmidt, R.J. Silage review: Interpretation of chemical, microbial, and organoleptic components of silages. J. Dairy Sci. 2018, 101, 4020–4033. [Google Scholar] [CrossRef] [Scilit]
- Da Silva, E.B.; Smith, M.L.; Savage, R.M.; Polukis, S.A.; Drouin, P.; Kung, L. Effects of Lactobacillus hilgardii 4785 and Lactobacillus buchneri 40788 on the bacterial community, fermentation and aerobic stability of high-moisture corn silage. J. Appl. Microbiol. 2021, 130, 1481–1493. [Google Scholar] [CrossRef] [Scilit]
- Bezerra, H.F.C.; Santos, E.M.; Oliveira, J.S.; Carvalho, G.G.P.; Pinho, R.M.A.; Silva, T.C.; Pereira, G.A.; Cassuce, M.R.; Zanine, A.M. Fermentation characteristics and chemical composition of elephant grass silage with ground maize and fermented juice of epiphytic lactic acid bacteria. S. Afr. J. Anim. Sci. 2019, 49, 522. [Google Scholar] [CrossRef] [Scilit]
- Matias, A.G.S.; Araujo, G.G.L.; Campos, F.S.; Moraes, S.A.; Gois, G.C.; Silva, T.S.; Emerenciano Neto, J.V.; Voltolini, T.V. Fermentation profile and nutritional quality of silages composed of cactus pear and maniçoba for goat feeding. J. Agric. Sci. 2020, 158, 304–312. [Google Scholar] [CrossRef] [Scilit]
- Silva, C.d.S.; de Miranda, A.S.; Novaes, J.J.d.S.; Araújo, C.d.A.; de Macedo, A.; de Araújo, J.S.; Lima, D.O.; Neto, J.V.E.; Gois, G.C.; de Araújo, G.G.L.; et al. Perfil fermentativo, valor nutricional e estabilidade aeróbia de silagens mistas de capim-elefante e cunhã. Ciência Anim. Bras. 2024, 25, e-76994. [Google Scholar] [CrossRef] [Scilit]
- Ferrero, F.; Piano, S.; Tabacco, E.; Borreani, G. Effects of conservation period and Lactobacillus hilgardii inoculum on the fermentation profile and aerobic stability of whole corn and sorghum silages. J. Sci. Food Agric. 2019, 99, 2530–2540. [Google Scholar] [CrossRef] [Scilit]
- Drouin, P.; Tremblay, J.; Renaud, J.; Apper, E. Microbiota succession during aerobic stability of maize silage inoculated with Lentilactobacillus buchneri NCIMB 40788 and Lentilactobacillus hilgardii CNCM-I-4785. Microbiol. Open 2021, 10, e1153. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ferrero, F.; Tabacco, E.; Borreani, G. Lentilactobacillus hilgardii Inoculum, Dry Matter Contents at Harvest and Length of Conservation Affect Fermentation Characteristics and Aerobic Stability of Corn Silage. Front. Microbiol. 2021, 12, 675563. [Google Scholar] [CrossRef] [Scilit]
- Arriola, K.G.; Vyas, D.; Kim, D.; Agarussi, M.C.N.; Silva, V.P.; Flores, M.; Jiang, Y.; Xue, Y.; Pech-Cervantes, A.A.; Ferraretto, L.F.; et al. Effect of Lactobacillus hilgardii, Lactobacillus buchneri, or their combination on the fermentation and nutritive value of sorghum silage and corn silage. J. Dairy Sci. 2021, 104, 9664–9675. [Google Scholar] [CrossRef] [Scilit]
- Araújo, V.L.; Rodriguez, N.M.; Gonçalves, L.C.; Rodrigues, J.A.S.; Borges, I.; Borges, A.L.C.C.; Saliba, E.O.S. Qualidade das silagens de três híbridos de sorgo ensilados em cinco diferentes estádios de maturação. Arq. Bras. Med. Veterinária Zootec. 2007, 59, 168–174. [Google Scholar] [CrossRef] [Scilit]
- Liu, B.; Huan, H.; Gu, H.; Xu, N.; Shen, Q.; Ding, C. Dynamics of a microbial community during ensiling and upon aerobic exposure in lactic acid bacteria inoculation-treated and untreated barley silages. Bioresour. Technol. 2019, 273, 212–219. [Google Scholar] [CrossRef] [Scilit]
- Xu, D.; Ding, W.; Ke, W.; Li, F.; Zhang, P.; Guo, X. Modulation of Metabolome and Bacterial Community in Whole Crop Corn Silage by Inoculating Homofermentative Lactobacillus plantarum and Heterofermentative Lactobacillus buchneri. Front. Microbiol. 2019, 9, 3299. [Google Scholar] [CrossRef] [Scilit]
- Association of Official Analytical Chemistry—AOAC International. Official Methods of Analysis of AOAC International, 15th ed.; Association of Official Analytical Chemistry—AOAC International: Arlington, VA, USA, 1990. [Google Scholar]
- Van Soest, P.J.; Robertson, J.B.; Lewis, B.A. Methods for Dietary Fiber, Neutral Detergent Fiber, and Nonstarch Polysaccharides in Relation to Animal Nutrition. J. Dairy Sci. 1991, 74, 3583–3597. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bolsen, K.K.; Lin, C.; Brent, B.E.; Feyerherm, A.M.; Urban, J.E.; Aimutis, W.R. Effect of Silage Additives on the Microbial Succession and Fermentation Process of Alfalfa and Corn Silages. J. Dairy Sci. 1992, 75, 3066–3083. [Google Scholar] [CrossRef] [Scilit]
- Dubois, M.; Gilles, K.A.; Hamilton, J.K.; Rebers, P.A.; Smith, F. Colorimetric Method for Determination of Sugars and Related Substances. Anal. Chem. 1956, 28, 350–356. [Google Scholar] [CrossRef] [Scilit]
- Siegfried, V.R.; Ruckemann, H.; Stumpf, G. Eine HPLC-methode zur bestimmung organischer säuren in silagen. Landwirtsch. Forsch. 1984, 37, 298–304. [Google Scholar]
- American Public Health Association. Compendium of Methods for the Microbiological Examination of Foods, 5th ed.; Salfinger, Y., Tortorello, M.L., Eds.; American Public Health Association (APHA): Washington, DC, USA, 2015. [Google Scholar]
- Kung, L.; Savage, R.M.; da Silva, E.B.; Polukis, S.A.; Smith, M.L.; Johnson, A.C.B.; Miller, M.A. The effects of air stress during storage and low packing density on the fermentation and aerobic stability of corn silage inoculated with Lactobacillus buchneri 40788. J. Dairy Sci. 2021, 104, 4206–4222. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Magalhães, F.A.; Valadares Filho, S.C.; Menezes, G.C.C.; Machado, M.G.; Zanetti, D.; Pina, D.S.; Pereira, O.G.; Paulino, M.F. Chemical composition and fermentative losses of sugar cane ensilage with different Brix degrees, with or without calcium oxide. Rev. Bras. Zootec. 2012, 41, 256–263. [Google Scholar] [CrossRef] [Scilit]
- Callahan, B.J.; McMurdie, P.J.; Rosen, M.J.; Han, A.W.; Johnson, A.J.A.; Holmes, S.P. DADA2: High-resolution sample inference from Illumina amplicon data. Nat. Methods 2016, 13, 581–583. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bolyen, E.; Rideout, J.R.; Dillon, M.R.; Bokulich, N.A.; Abnet, C.C.; Al-Ghalith, G.A.; Alexander, H.; Alm, E.J.; Arumugam, M.; Asnicar, F.; et al. Reproducible, interactive, scalable and extensible microbiome data science using QIIME 2. Nat. Biotechnol. 2019, 37, 852–857. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Quast, C.; Pruesse, E.; Yilmaz, P.; Gerken, J.; Schweer, T.; Yarza, P.; Peplies, J.; Glöckner, F.O. The SILVA ribosomal RNA gene database project: Improved data processing and web-based tools. Nucleic Acids Res. 2013, 41, D590–D596. [Google Scholar] [CrossRef] [Scilit]
- Nilsson, R.H.; Larsson, K.H.; Taylor, A.F.S.; Bengtsson-Palme, J.; Jeppesen, T.S.; Schigel, D.; Kennedy, P.; Picard, K.; Glöckner, F.O.; Tedersoo, L.; et al. The UNITE database for molecular identification of fungi: Handling dark taxa and parallel taxonomic classifications. Nucleic Acids Res. 2019, 47, D259–D264. [Google Scholar] [CrossRef] [Scilit]
- McMurdie, P.J.; Holmes, S. phyloseq: An R Package for Reproducible Interactive Analysis and Graphics of Microbiome Census Data. PLoS ONE 2013, 8, e61217. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lozupone, C.A.; Knight, R. The unifrac significance test is sensitive to tree topology. BMC Bioinform. 2015, 16, 211. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gilmore, R.; Hutchins, S.; Zhang, X.; Vallender, E. MicrobiomeR: An R Package for Simplified and Standardized Microbiome Analysis Workflows. J. Open-Source Softw. 2019, 4, 1299. [Google Scholar] [CrossRef] [Scilit]
- Ferreira, D.F. SISVAR: A computer analysis system to fixed effects split plot type designs. Rev. Bras. Biom. 2019, 37, 529–535. [Google Scholar] [CrossRef] [Scilit]
- Love, M.I.; Huber, W.; Anders, S. Moderated estimation of fold change and dispersion for RNA-seq data with DESeq2. Genome Biol. 2014, 15, 550. [Google Scholar] [CrossRef] [Scilit]
- Segata, N.; Izard, J.; Waldron, L.; Gevers, D.; Miropolsky, L.; Garrett, W.S.; Huttenhower, C. Metagenomic biomarker discovery and explanation. Genome Biol. 2011, 12, R60. [Google Scholar] [CrossRef] [Scilit]
- Xu, R.; Zhao, H.; You, Y.; Wu, R.; Liu, G.; Sun, Z.; Bademuqiqige; Zhang, Y. Effects of Intercropping, Nitrogen Fertilization and Corn Plant Density on Yield, Crude Protein Accumulation and Ensiling Characteristics of Silage Corn Interseeded into Alfalfa Stand. Agriculture 2022, 12, 357. [Google Scholar] [CrossRef] [Scilit]
- Xu, H.; Wu, N.; Na, N.; Ding, H.; Sun, L.; Fang, Y.; Li, D.; Li, E.; Yang, B.; Wei, X.; et al. Dynamics of fermentation quality, bacterial communities, and fermentation weight loss during fermentation of sweet sorghum silage. BMC Microbiol. 2024, 24, 429. [Google Scholar] [CrossRef] [Scilit]
- Heinl, S.; Wibberg, D.; Eikmeyer, F.; Szczepanowski, R.; Blom, J.; Linke, B.; Goesmann, A.; Grabherr, R.; Schwab, H.; Pühler, A.; et al. Insights into the completely annotated genome of Lactobacillus buchneri CD034, a strain isolated from stable grass silage. J. Biotechnol. 2012, 161, 153–166. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ávila, C.L.S.; Carvalho, B.F.; Pinto, J.C.; Duarte, W.F.; Schwan, R.F. The use of Lactobacillus species as starter cultures for enhancing the quality of sugar cane silage. J. Dairy Sci. 2014, 97, 940–951. [Google Scholar] [CrossRef] [Scilit]
- Fernandes, T.; Paula, E.M.; Sultana, H.; Ferraretto, L.F. Short communication: Influence of sorghum cultivar, ensiling storage length, and microbial inoculation on fermentation profile, N fractions, ruminal in situ starch disappearance and aerobic stability of whole-plant sorghum silage. Anim. Feed Sci. Technol. 2020, 266, 114535. [Google Scholar] [CrossRef] [Scilit]
- Gomes, A.L.M.; Bueno, A.V.I.; Osmari, M.P.; Machado, J.; Nussio, L.G.; Jobim, C.C.; Daniel, J.L.P. Effects of Obligate Heterofermentative Lactic Acid Bacteria Alone or in Combination on the Conservation of Sugarcane Silage. Front. Microbiol. 2021, 12, 643879. [Google Scholar] [CrossRef] [Scilit]
- Zhang, L.; Zhou, X.; Gu, Q.; Liang, M.; Mu, S.; Zhou, B.; Huang, F.; Lin, B.; Zou, C. Analysis of the correlation between bacteria and fungi in sugarcane tops silage prior to and after aerobic exposure. Bioresour. Technol. 2019, 291, 121835. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhao, S.; Yang, F.; Wang, Y.; Fan, X.; Feng, C.; Wang, Y. Dynamics of Fermentation Parameters and Bacterial Community in High-Moisture Alfalfa Silage with or without Lactic Acid Bacteria. Microorganisms 2021, 9, 1225. [Google Scholar] [CrossRef] [Scilit]
- Silva, N.C.; Nascimento, C.F.; Nascimento, F.A.; de Resende, F.D.; Daniel, J.L.P.; Siqueira, G.R. Fermentation and aerobic stability of rehydrated corn grain silage treated with different doses of Lactobacillus buchneri or a combination of Lactobacillus plantarum and Pediococcus acidilactici. J. Dairy Sci. 2018, 101, 4158–4167. [Google Scholar] [CrossRef] [Scilit]
- Tavares, B.C.; Dias, M.; Royer, J.L.; Nascimento, V.A.; Dias, F.J.d.S.; Saenz, E.A.C.; Câmara, L.R.d.A.; da Silveira, D.M. Doses de inoculante bacteriano Lentilactobacillus buchneri NCIMB 40788 na silagem de grão de milho reidratado. Cuad. Educ. Desarro. 2024, 16, e6339. [Google Scholar] [CrossRef] [Scilit]
- Junges, D.; Morais, G.; Spoto, M.H.F.; Santos, P.S.; Adesogan, A.T.; Nussio, L.G.; Daniel, J.L.P. Short communication: Influence of various proteolytic sources during fermentation of reconstituted corn grain silages. J. Dairy Sci. 2017, 100, 9048–9051. [Google Scholar] [CrossRef] [Scilit]
- dos Santos, A.C.P.; Santos, E.M.; Carvalho, G.G.P.; Perazzo, A.F.; Araújo, M.L.G.M.L.; de Oliveira, J.S.; Pereira, G.A.; Macêdo, A.J.d.S.; Sá, W.C.C.d.S.; Pereira, D.M. Fermentation profile, microbial populations and aerobic stability of sorghum silages enriched with urea and Lactobacillus buchneri. N. Z. J. Agric. Res. 2021, 66, 128–144. [Google Scholar] [CrossRef] [Scilit]
- de L. Nascimento, M.E.; Edvan, R.L.; Santos, E.M.; de Oliveira, J.S.; de S. Miranda, R.; Nascimento, R.R.D.; de S. Barros, L.; de Oliveira, C.J.B.; de S. Santos, F.N.; Pereira, D.M.; et al. Effect of Lactobacillus buchneri and sodium benzoate on the fermentative profile, bacterial taxonomic diversity, and aerobic stability of sorghum silages at different fermentation times. Chil. J. Agric. Res. 2023, 83, 539–552. [Google Scholar] [CrossRef] [Scilit]
- Li, X.; Cheng, Y.; Yang, F.; Hu, J.; Ma, R.; Liu, H.; Shao, T. Improving Total Mixed Ration Silage: Effects of Lactic Acid Bacteria Inoculants and Antimicrobial Additives on Fermentation Quality and Aerobic Stability. Agronomy 2024, 14, 1602. [Google Scholar] [CrossRef] [Scilit]
- Drouin, P.; Tremblay, J.; Chaucheyras-Durand, F. Dynamic Succession of Microbiota during Ensiling of Whole Plant Corn Following Inoculation with Lactobacillus buchneri and Lactobacillus hilgardii Alone or in Combination. Microorganisms 2019, 7, 595. [Google Scholar] [CrossRef] [Scilit]
- Kleinschmit, D.H.; Kung, L. A Meta-Analysis of the Effects of Lactobacillus buchneri on the Fermentation and Aerobic Stability of Corn and Grass and Small-Grain Silages. J. Dairy Sci. 2006, 89, 4005–4013. [Google Scholar] [CrossRef] [Scilit]
- Oliveira, A.S.; Weinberg, Z.G.; Ogunade, I.M.; Cervantes, A.A.P.; Arriola, K.G.; Jiang, Y.; Kim, D.; Li, X.; Gonçalves, M.C.M.; Vyas, D.; et al. Meta-analysis of effects of inoculation with homofermentative and facultative heterofermentative lactic acid bacteria on silage fermentation, aerobic stability, and the performance of dairy cows. J. Dairy Sci. 2017, 100, 4587–4603. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Morais, L.B.; Carvalho, B.F.; Batista, L.R.; Schwan, R.F.; Ávila, C.L.S. Mycological diversity in whole-plant corn silages inoculated with Lentilactobacillus buchneri or Lentilactobacillus farraginis. Arq. Bras. Med. Veterinária Zootec. 2024, 76, 114–130. [Google Scholar] [CrossRef] [Scilit]
- Wang, C.; Han, H.; Sun, L.; Na, N.; Xu, H.; Chang, S.; Jiang, Y.; Xue, Y. Bacterial Succession Pattern during the Fermentation Process in Whole-Plant Corn Silage Processed in Different Geographical Areas of Northern China. Processes 2021, 9, 900. [Google Scholar] [CrossRef] [Scilit]
- Korcari, D.; Ricci, G.; Capusoni, C.; Fortina, M.G. Physiological performance of Kazachstania unispora in sourdough environments. World J. Microbiol. Biotechnol. 2021, 37, 88. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Borreani, G.; Tabacco, E.; Schmidt, R.J.; Holmes, B.J.; Muck, R.E. Silage review: Factors affecting dry matter and quality losses in silages. J. Dairy Sci. 2018, 101, 3952–3979. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Reis, C.B.; Santos, A.d.O.d.; Carvalho, B.F.; Schwan, R.F.; Ávila, C.L.d.S. Wild Lactobacillus hilgardii (CCMA 0170) strain modifies the fermentation profile and aerobic stability of corn silage. J. Appl. Anim. Res. 2018, 46, 632–638. [Google Scholar] [CrossRef] [Scilit]
- Alves, W.S.; Pereira, O.G.; Macêdo, A.J.d.S.; Leite, G.D.O.; da Silva, V.P.; Leite, P.S.; Ribeiro, K.G.; Filho, S.d.C.V. Effect of new strains of Lentilactobacillus buchneri as inoculants in sorghum silage on the fermentative profile, aerobic stability, and voluntary intake in lambs. N. Z. J. Agric. Res. 2025, 68, 613–629. [Google Scholar] [CrossRef] [Scilit]
- Shahrajabian, M.H.; Sun, W. The Significance and Importance of dPCR, qPCR, and SYBR Green PCR Kit in the Detection of Numerous Diseases. Curr. Pharm. Des. 2024, 30, 169–179. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.