


Abstract
Leg-spring hysteresis, the mechanical energy dissipated within the force–length loop during ground contact, is a whole-limb, indirect indicator of stretch-shortening cycle (SSC) function. Whether international-level track-and-field and club-level multi-sport athletes differ in hysteresis responses to drop height, and whether hysteresis is associated with jump height, remains unclear. Here, 40 athletes (15 international-level, 25 club-level) performed bilateral (BLJ), dominant-leg (DOM), and non-dominant-leg (NDOM) drop jumps from 0.26 to 0.42 m. Hysteresis and jump height were computed from three-dimensional kinematics (500 Hz) and ground reaction forces. Group × drop-height interactions were significant for hysteresis in all conditions (partial eta-squared, η2p = 0.647, 0.507, 0.466; p < 0.001): international-level athletes became increasingly negative (net active energy contribution) at 0.42 m, whereas club-level athletes became positive (net dissipation). Between-group differences at 0.42 m were large (Cohen’s d = −1.73, DOM; −1.95, NDOM); jump height was also higher in international-level athletes (d = 1.14–1.77). Pooled, hysteresis was associated with jump height (coefficient of determination, R2 = 0.44–0.60), although caliber differences inflate this estimate, and within-group associations were weaker. Hysteresis discriminated reactive-jumping capacity beyond jump height alone; because competitive level was confounded with sport discipline and sex, these differences should not be attributed to caliber per se.
1. Introduction
The spring-mass model provides a productive mechanical framework for characterizing lower-extremity behavior during bouncing gaits and reactive-jumping tasks [1,2]. Within this framework, the lower limb is idealized as a massless spring, whose compression and recoil during ground contact govern the energetics of the stance phase. Leg-spring stiffness, defined as the ratio of the peak vertical ground reaction force to the maximum leg compression, has been consistently associated with running economy, jump height, and sprint performance across diverse athletic populations [3,4,5]. However, stiffness alone does not fully characterize the elastic energy storage and return cycles. An idealized spring recovers all stored strain energy upon unloading, whereas biological musculotendinous tissues inevitably dissipate a proportion of mechanical energy through viscoelastic damping [6,7]. At the tissue level, in vivo human tendons exhibit mechanical hysteresis of approximately 18% under physiological loading, reflecting the inherent viscoelastic behavior of collagenous structures [8]. Critically, longitudinal evidence has demonstrated that 12 weeks of plyometric training significantly reduces tendon hysteresis during ballistic contractions while concurrently increasing active muscle stiffness and jump performance, indicating that the efficiency of elastic energy return is a trainable mechanical property [9]. At the whole-limb level, hysteresis is quantified from the force–length loop traced by the leg spring during ground contact, as the signed difference between the mechanical energy absorbed during the braking (loading) phase and the energy returned during the propulsion (unloading) phase, expressed relative to the energy absorbed [10,11]. A strictly passive viscoelastic spring returns less energy than it absorbs and, therefore, yields positive hysteresis (net dissipation); in an active musculotendinous system, concentric muscle work performed during propulsion can return more mechanical energy than was absorbed during braking, reversing the orientation of the loop and producing negative hysteresis, a whole-limb mechanical pattern consistent with greater active contribution during unloading [10,11]. The sign convention and its computation are detailed in Section 2.4 and illustrated in Figure 1.
Figure 1.
Schematic of the leg-spring force–length loop and the hysteresis sign convention. Ground reaction force is plotted against leg length during ground contact (touchdown at the longest leg length; the leg shortens toward the left); the solid curve denotes the loading (braking) branch and the dashed curve the unloading (propulsion) branch, with arrows indicating the direction of loop traversal. The shaded region is the energy absorbed during loading (Aascending). (a) When the unloading branch lies below the loading branch (Aascending > Adescending), the loop is traversed clockwise, the unloading work is less than the loading work, and hysteresis is positive (net dissipation). (b) When concentric muscle work raises the unloading branch above the loading branch (Aascending < Adescending), the loop is traversed counterclockwise, the unloading work exceeds the loading work, and hysteresis is negative (net active energy contribution). Hysteresis (%) = (Aloop/Aascending) × 100, with Aloop = Aascending − Adescending. Curves are illustrative and not drawn from measured data.
The stretch-shortening cycle (SSC) is defined as a rapid sequence of eccentric loading and concentric unloading of the musculotendinous unit, during which the elastic strain energy stored in the series elastic components is recovered to augment propulsive force output [7,12,13]. Pre-activation of the relevant musculature before ground contact, precise timing of the eccentric-to-concentric transition, and adequate musculotendinous stiffness are necessary conditions for effective elastic energy return [14]. Drop-jump tasks operationalize these requirements by imposing a controlled eccentric loading stimulus whose magnitude scales with drop height, rendering them a validated and widely employed paradigm for probing SSC mechanics across various performance levels [11,15,16]. A recent systematic review and meta-analysis confirmed that the reactive strength index (RSI) is meaningfully associated with independent markers of athletic performance [17], and plyometric jump training reliably improves RSI across diverse athlete populations [18]. International-level athletes generally demonstrate shorter ground contact times and superior RSI values compared with recreationally trained or club-level populations [4,15], although expertise-related differences in leg-spring stiffness itself have not been consistently reported [16]; such differences are attributable in part to long-term plyometric training adaptations [9,19]. Despite this body of evidence, whether international-level track-and-field athletes and club-level multi-sport athletes differ in their hysteresis responses to systematically increasing drop heights and whether such differences predict jump performance remains unknown.
Therefore, this study addressed three primary aims: (i) to compare leg-spring hysteresis and jump height between groups across bilateral (BLJ), dominant-leg (DOM), and non-dominant-leg (NDOM) drop-jump conditions performed from two systematically varied drop heights; (ii) to determine whether a significant group × drop-height interaction existed for hysteresis and jump height; and (iii) to quantify the predictive validity of hysteresis for jump height at 0.42 m. It was hypothesized that (H1) international-level athletes would exhibit markedly lower (more negative) hysteresis values at 0.42 m relative to 0.26 m, a pattern consistent with greater net active contribution during the unloading phase; (H2) a significant group × drop-height interaction would emerge for hysteresis across all three jump conditions; and (H3) hysteresis would be significantly associated with jump height at 0.42 m.
2. Materials and Methods
2.1. Participants
In this study, 40 athletes participated, comprising 15 international-level track-and-field athletes (5 females, 10 males) and 25 club-level multi-sport athletes (15 females, 10 males). Demographic and anthropometric characteristics are presented in Table 1. The two groups were well matched for height, body mass, and BMI. International-level athletes were significantly older than club-level athletes (U = 314.0, p < 0.001, d = 0.69). The dominant leg was operationally defined as the leg each athlete habitually used for single-leg take-off (jump-leg preference). The sex distribution did not differ significantly between groups (χ2(1) = 1.71, p = 0.191). The implications of sport discipline and sex distribution differences between groups are addressed in the sensitivity analyses (Section 3.3) and study limitations (Section 4.5).
Table 1.
Demographic and anthropometric characteristics by group.
International-level athletes were track-and-field competitors with at least five years of continuous competition experience who had competed at major international championships (European Athletics Championships or equivalent). The group included high jumpers (n = 2), triple jumpers (n = 1), shot put athletes (n = 1), hurdlers (n = 2), javelin throwers (n = 2), sprinters (n = 4), pole vaulters (n = 1), and long jumpers (n = 2). Club-level athletes included track-and-field athletes (n = 2), basketball players (n = 14), handball players (n = 2), and volleyball players (n = 7). All participants had a minimum of one year of structured plyometric or athletic training experience before data collection.
Participants were excluded if they had a history of lower-extremity surgery, current lower-extremity injury, or any musculoskeletal injury in the preceding 12 months. All participants provided written informed consent prior to testing. The study was approved by the Non-Interventional Clinical Research Ethics Committee (Approval No. 232; date: 30 November 2022). All procedures were conducted in accordance with the ethical standards of the Declaration of Helsinki (revised 2013).
2.2. Procedure
All athletes completed a standardized 10 min warm-up consisting of five minutes of light jogging, followed by five minutes of dynamic lower-extremity stretching. Submaximal countermovement jumps and familiarization drop jumps were subsequently performed. Participants were instructed to land on the forefoot and immediately perform a maximum-effort vertical jump, minimizing ground contact time while maximizing jump height [11,15]. Sixty-one retroreflective markers were placed on anatomical landmarks following a full-body marker set based on the Plug-in Gait convention, implemented in Visual3D (v6, C-Motion, Germantown, MD, USA). Following static calibration, 8 markers used exclusively for anatomical calibration were removed, leaving 53 tracking markers for the dynamic trials.
Participants performed bilateral drop jumps (BLJ), dominant-leg drop jumps (DOM), and non-dominant-leg drop jumps (NDOM) from two fixed drop heights: drop height 1 (0.26 m) and drop height 2 (0.42 m). These heights were selected to represent a low-to-moderate loading range consistent with prior drop-jump research [11,16]. The order of jump conditions and drop heights was fully counterbalanced across participants using Research Randomizer software (Version 4.0) [20]. Each participant completed three maximal trials per condition, and the trial producing the highest jump height was retained for analysis to capture each athlete’s actual maximal reactive capacity. The robustness of this selection strategy was confirmed through a mean-of-three-trials sensitivity analysis (see Section 2.4 and Section 3.8) [11]. Rest intervals of 60 s between trials and 2 min between conditions were enforced [15]. Participants stepped off the drop height without an initial upward or downward jump, so that the descent height corresponded to the prescribed drop height. Throughout every trial, the hands were kept on the hips to remove any contribution of arm swing to jump height and to keep the pelvic and lower-limb markers continuously visible to the motion capture cameras. All jumps were performed in each participant’s own athletic training footwear, which remained unchanged across all conditions and drop heights. A trial was discarded and repeated if the participant failed to land within the boundaries of the force platform, took an additional step on landing, or visibly paused between the landing and take-off phases.
2.3. Instrumentation and Data Capture
Three-dimensional kinematic data were collected at 500 Hz using seven Oqus 7+ infrared cameras (Qualisys Track Manager v2020.3; Qualisys AB, Gothenburg, Sweden). Ground reaction forces (GRFs) were recorded synchronously at 500 Hz using a six-component force platform (Bertec FP6090-15-TM; Bertec Corporation, Columbus, OH, USA). Kinematic data were filtered using a fourth-order, zero-lag, dual-pass Butterworth low-pass filter with a cutoff frequency of 12 Hz. Kinetic (GRF) data were left unfiltered prior to calculation of leg-spring stiffness and hysteresis to prevent artificial attenuation of the impact transient. The 500 Hz acquisition rate yields a Nyquist frequency of 250 Hz, which exceeds the frequency band carrying the majority of the signal power in drop-landing ground reaction forces; because the primary outcome is the enclosed area of the force–length loop—an integrated work quantity governed by the low-frequency envelope of the force–length trajectory rather than by the highest-frequency components of the impact spike—the hysteresis estimates are comparatively robust to modest undersampling of the transient peak, although a higher rate would resolve the instantaneous peak force more sharply. The 500 Hz acquisition rate, therefore, provides sufficient resolution for robust whole-limb energy calculations. Because leg length was derived from low-pass-filtered kinematics whereas force was retained unfiltered, the two axes of the force–length loop were not subjected to identical frequency conditioning, which may introduce a small distortion of the computed loop area during the early braking phase. To ensure the robustness of the findings against the filtering asymmetry, we compared unfiltered GRF with variants filtered at 12, 50, and 100 Hz (Supplementary Table S1). Hysteresis estimates were remarkably stable across all filtering conditions, with a maximum mean difference of less than 2.5% between filtered and unfiltered versions, and the qualitative distinction between groups (negative versus positive hysteresis) remained invariant regardless of the GRF cutoff frequency. All data were processed using Visual3D (v6, C-Motion) to generate rigid-body segment models and compute whole-body center-of-mass (COM) trajectories. The hip joint center (HJC) was estimated using the regression method of Bell et al. [21]. To minimize any potential phase-shift discrepancy between the filtered kinematics (12 Hz low-pass) and unfiltered GRF data, the touchdown and take-off events used to partition the loop branches were strictly synchronized using the unfiltered force threshold (20 N) in the time domain, protecting the loop area calculations from artificial phase distortions.
2.4. Data Analysis
Jump height was calculated from the vertical displacement of the whole-body COM between take-off and the apex of the flight phase. Leg length was defined as the absolute (non-normalized) three-dimensional Euclidean distance between the HJC and the instantaneous center of pressure; no reference-length subtraction or normalization was applied, so all force–length loops were expressed in terms of absolute leg length rather than leg compression relative to a reference configuration. Defining leg length as the instantaneous distance between the HJC and the COP accounts for the dynamic translation of the center of pressure during ground contact; although COP translation introduces minor non-axial displacement, this approach provides a robust representation of the virtual leg-spring length in biological systems, in line with established spring-mass modeling protocols [4,10,11]. Where used, leg compression denotes the corresponding reduction in leg length relative to the touchdown configuration. Leg-spring stiffness (k) was computed as the slope of a linear ordinary least-squares regression fitted to the loading-phase force–length curve [5,11]. Hysteresis was quantified from the force–length loop as follows.
For each contact, the force–length loop was constructed by plotting the ground reaction force projected onto the leg-spring axis (the line joining the HJC and the center of pressure) against instantaneous leg length from touchdown to take-off and was partitioned at the instant of maximum leg compression into a loading (braking) branch and an unloading (propulsion) branch. The energy absorbed during loading (Aascending) and the energy returned during unloading (Adescending) were each computed as the magnitude of the work integral ∫F dL along the respective branch, evaluated numerically by the trapezoidal rule, with the signed enclosed loop area defined as Aloop = Aascending − Adescending:
Hysteresis (%) = (Aloop/Aascending) × 100
Positive values arise when the unloading branch lies below the loading branch (Adescending < Aascending), indicating net energy dissipation, as expected of a passive viscoelastic spring; negative values arise when the unloading branch lies above the loading branch (Adescending > Aascending), indicating that concentric muscle work returned more mechanical energy than was absorbed during braking—a net whole-limb mechanical work outcome during propulsion, in which the unloading work exceeds the loading work [10,11]. The two cases are illustrated schematically in Figure 1. Methodological note: Leg-spring hysteresis is derived from whole-limb force–length loop kinematics and kinetics, not from direct measurement of tendon or muscle fascicle behavior; therefore, the magnitude and sign of hysteresis should be interpreted as a whole-limb mechanical proxy rather than as direct evidence of tissue-level elastic energy storage or retrieval without supporting ultrasonographic or electromyographic evidence. Because the leg spring in a maximal drop jump is an actively powered actuator rather than a passive elastic element, negative whole-limb hysteresis is not bounded at −100%; values beyond this bound are mathematically admissible and denote propulsion-phase work exceeding braking-phase work by more than 100%. Such values quantify net whole-limb mechanical work during propulsion and, unlike tendon-level hysteresis (approximately 18% measured in vivo) [8], do not carry an upper physiological ceiling on the negative side.
Between-group comparisons were conducted using independent-samples t-tests or Mann–Whitney U tests as appropriate based on Shapiro–Wilk normality testing; for all independent-samples t-tests, Welch’s correction was applied because group sizes were unequal and variances heterogeneous across several conditions, so degrees of freedom are reported as non-integer values. To account for the within-participant dependency across the repeated bilateral and unilateral conditions and to limit the number of separate tests, the primary omnibus analysis of hysteresis and jump height used a linear mixed-effects model with group, drop height, condition, and all interactions as fixed effects and a by-participant random intercept, estimated by restricted maximum likelihood. Fixed effects were evaluated using Type III Wald chi-square tests (χ2), which in the SPSS Version 29.0 MIXED procedure are computed as the square of the ratio of each parameter estimate to its standard error (z2 = χ2(1)); this notation is used consistently throughout the results. All linear mixed-effects models were estimated using the MIXED procedure in IBM SPSS Statistics (version 29.0; IBM Corp., Armonk, NY, USA), with restricted maximum likelihood (REML) estimation. Categorical predictors were dummy-coded with the following reference levels: group (club-level = 0, international-level = 1), sex (female = 0, male = 1), drop height (0.26 m = 0, 0.42 m = 1), and condition (BLJ = reference; DOM and NDOM contrasted against BLJ). Standardized estimates (β), therefore, quantify the deviation of each active level from its respective reference category. The condition-specific 2 × 2 (group × drop height) ANOVAs and their partial eta-squared values are retained as descriptive decompositions of the interaction. Hierarchical regression models predicting jump height from hysteresis were constructed in two steps: a linear model (Step 1), followed by the addition of a quadratic term (Step 2). Leg-spring stiffness was entered as a second predictor in exploratory Step 3. To distinguish a within-level association from between-cohort separation, each 0.42 m model was additionally re-estimated with group as a covariate (group-adjusted model) and with a group × hysteresis interaction term; the incremental variance attributable to hysteresis beyond group (ΔR2) and the group-specific slopes were computed. To examine whether demographic variance accounted for the observed effects, chronological age (continuous covariate) and sex (fixed factor) were additionally entered into the linear mixed-effects models for leg-spring hysteresis and for jump height; these adjusted models indicate the extent to which the observed mechanical differences track athletic caliber (group) rather than age or sex. These adjusted models retained group, drop height, condition, age and sex as fixed effects together with the group × drop-height interaction but did not include the higher-order condition interactions; the group × drop-height term, therefore, not numerically identical to the corresponding term in the unadjusted model. Model intercepts are constants of the fitted equations and are not interpreted substantively. The contribution of sex was additionally examined with a two-way factorial ANOVA (general linear model) with group and sex as between-subjects fixed factors and their interaction, computed separately for each jump condition at the 0.42 m drop height (Section 3.3). Age was an admissible covariate in these models because it varied within both groups with overlapping distributions. Sport discipline was fully confounded with group and could not be modelled. Sex, however, varied within both groups and was, therefore, examined through sex-stratified descriptive statistics, a group contrast restricted to the sex-balanced male stratum (Section 3.3), and as a fixed factor in the adjusted mixed-effects models (Section 3.5); the residual confounding is addressed as a design limitation (Section 4.5). Because multiple inferential tests were conducted, interpretation emphasizes the magnitude and cross-condition consistency of effects rather than the significance of any single comparison; no familywise correction was applied, and the exploratory analyses (Section 3.3 and Section 3.4) are identified as such. Effect sizes were reported as Cohen’s d (between-group comparisons), η2p (ANOVA interactions), and Pearson r (bivariate associations) [22]. Intra-session reliability for hysteresis and jump height was quantified using the Intraclass Correlation Coefficient (ICC) and Coefficient of Variation (CV%) across all three recorded trials per participant, employing a two-way mixed-effects, single-measurement, absolute-agreement model (McGraw–Wong ICC(A,1) terminology) [23]; because the primary analyses used the single best (highest) trial per condition rather than the across-trial mean, these coefficients characterize the trial-to-trial consistency of the measurement rather than the precision of the specific maximal value retained for analysis. Because hysteresis values frequently approach or cross zero (inflating CV%), the absolute Standard Error of Measurement (SEM = SDpooled × √(1 − ICC)) was calculated for hysteresis instead. All statistical analyses were performed using IBM SPSS Statistics (version 29.0; IBM Corp., Armonk, NY, USA). Because the sample size was fixed by athlete availability, a sensitivity analysis was conducted in G*Power (version 3.1.9.7) [24] to establish the smallest effects the design could reliably detect rather than to estimate post hoc observed power. With α = 0.05 and power = 0.80 and the realized group sizes (n = 15 and n = 25), the minimum detectable effect was Cohen’s d = 0.94 for the between-group comparisons and partial η2 = 0.17 (Cohen’s f = 0.46) for a single-degree-of-freedom F test, the latter serving as a conservative reference for both the group × drop-height interaction and the single-predictor regression; the primary effects reported below (|d| = 1.14–1.95; interaction η2p = 0.47–0.65; regression R2 = 0.44–0.60) substantially exceeded these thresholds, whereas smaller effects could not be reliably detected, so non-significant findings are interpreted as inconclusive rather than as evidence of absence. To verify the mathematical stability of the computed hysteresis values and rule out selection or measurement bias, a methodological sensitivity analysis was conducted. Hysteresis and stiffness parameters were re-calculated using two distinct kinematics-tracking models: the Center of Mass (CoM) reference model and the hip joint center (HJC) reference model. Pearson correlation coefficients and group interaction effects were compared across both models to confirm the robustness of the primary findings.
3. Results
3.1. Reliability of Hysteresis and Jump Height
Intra-session reliability for jump height was excellent across all conditions, with ICC(A,1) values ranging from 0.94 to 0.98 and CV% ranging from 3.2% to 5.8%. For leg-spring hysteresis, reliability was good to excellent, with ICC(A,1) values ranging from 0.85 to 0.92 [23]. The SEM for hysteresis ranged from 8.5% to 12.4%, indicating acceptable trial-to-trial measurement stability. Crucially, the observed between-group differences in hysteresis at 0.42 m (international-level: −49.67% vs. club-level: +1.00%; absolute difference ≈ 51 percentage points) exceeded the largest SEM observed in any condition (12.4%) by a factor of approximately four and the SEM for the corresponding bilateral 0.42 m condition (8.5%) by a factor of approximately six, supporting the interpretation that the observed group differences exceeded the expected measurement error (Table 2).
Table 2.
Intra-session reliability metrics for jump height and leg-spring hysteresis across all drop-jump conditions (n = 40).
3.2. Between-Group Comparisons of Hysteresis and Jump Height
Between-group comparisons of leg-spring hysteresis are summarized in Table 3. At the 0.26 m drop height, the two groups did not differ significantly in any condition (bilateral, U = 205.0, p = 0.635, d = −0.01; dominant-leg, t(33.3) = 1.85, p = 0.074, d = 0.50; non-dominant-leg, t(38.0) = 1.05, p = 0.302, d = 0.30), and both exhibited comparably negative hysteresis. At the 0.42 m drop height, by contrast, the groups diverged sharply in all three conditions, with very large effect sizes: international-level athletes displayed strongly negative hysteresis, whereas club-level athletes shifted to near-zero or net-positive values (bilateral, −49.67 ± 32.44% vs. 1.00 ± 25.74%, U = 30.0, p < 0.001, d = −1.78; dominant-leg, −28.37 ± 25.31% vs. 21.35 ± 30.61%, t(34.1) = −5.55, p < 0.001, d = −1.73; non-dominant-leg, −28.15 ± 32.40% vs. 19.72 ± 18.50%, t(19.6) = −5.23, p < 0.001, d = −1.95). The between-group separation in hysteresis was, therefore, height-dependent, emerging only under the more demanding eccentric load (Table 3).
Table 3.
Between-group comparison of leg-spring hysteresis (%) by condition and drop height.
Between-group comparisons of jump height are presented in Table 4. In contrast to the height-dependent hysteresis pattern, international-level athletes jumped significantly higher than club-level athletes in every condition at both drop heights, with large effect sizes throughout (d = 1.14–1.77). At 0.26 m, the differences were significant for the bilateral (0.313 ± 0.065 m vs. 0.209 ± 0.055 m, t(25.8) = 5.18, p < 0.001, d = 1.77), dominant-leg (0.147 ± 0.056 m vs. 0.095 ± 0.034 m, t(20.3) = 3.25, p = 0.004, d = 1.21), and non-dominant-leg conditions (0.148 ± 0.056 m vs. 0.098 ± 0.036 m, t(21.0) = 3.10, p = 0.005, d = 1.14), and they remained significant in all three conditions at 0.42 m (bilateral, p = 0.005, d = 1.17; dominant-leg, p = 0.002, d = 1.26; non-dominant-leg, p = 0.007, d = 1.14). Jump height, thus, distinguished the groups uniformly across loading conditions, whereas hysteresis distinguished them only at the higher drop height—a dissociation examined further in Section 3.5 and Section 4.2 (Table 4).
Table 4.
Between-group comparison of jump height (m) by condition and drop height.
3.3. Sensitivity Analyses: Within-Group Discipline Comparison and Age and Sex Adjustment
The international-level group comprised athletes from disciplines with divergent demands on lower-extremity SSC mechanics, permitting a limited test of whether the negative-hysteresis signature was specific to a single discipline within the elite cohort. An exploratory within-group comparison for the 0.42 m bilateral drop-jump condition indicated that elastic specialists (jumpers, sprinters, and hurdlers; n = 12) and throwing athletes (shot put and javelin; n = 3) both exhibited strongly negative hysteresis (−46.06 ± 28.94% and −63.81 ± 48.85%, respectively); the throwing subgroup achieved substantially lower bilateral jump height (0.261 ± 0.129 m) compared to elastic specialists (0.311 ± 0.063 m). Because the throwing subgroup was very small (n = 3), this comparison is illustrative only and was not subjected to inferential testing; it indicates that the negative-hysteresis pattern was present across mechanically dissimilar track-and-field disciplines rather than confined to elastic-recoil specialists. Because age was partly confounded with group, covariate adjustment alone cannot be regarded as decisive: partialling out a covariate that covaries with the grouping factor removes group-relevant variance and yields estimates that require cautious interpretation [25]. The role of age was, therefore, evaluated by two complementary routes: within-group correlations, which require no adjustment, and formal adjustment within the mixed-effects models reported in Section 3.5. Within neither group did age predict 0.42 m hysteresis in any condition (international: r = −0.29 to −0.43, all p ≥ 0.11; club: r = +0.12 to +0.22, all p ≥ 0.29), whereas the pooled correlation was significant (r = −0.36 to −0.40, all p < 0.05). The pooled age–hysteresis association, therefore, arises entirely from between-group separation rather than from any within-athlete dependency, indicating that the older mean age of the international-level group cannot account for its more negative hysteresis (Section 4.5).
Because the sex distribution was unequal between groups (international: 10 M/5 F; club: 10 M/15 F), 0.42 m hysteresis was additionally summarized by sex within each group (Table 5), and individual hysteresis values disaggregated by sex and sport discipline are shown in Supplementary Figure S1, which confirms that the negative-hysteresis signature of the international-level group was present in both sexes and across track-and-field disciplines, including the throwing subgroup. The international-versus-club difference persisted within both sexes and, importantly, within the sex-balanced male stratum (10 vs. 10), where international-level males remained strongly negative and club-level males clustered near zero to positive (BLJ d = −1.52; DOM d = −1.37; NDOM d = −1.77); differences within females were of comparable or larger magnitude (d = −1.97 to −2.84). Within groups, males tended toward more negative hysteresis than females (international d(M−F) = −0.73 to −0.86; club d = −0.05 to −0.95), a smaller effect that did not reverse the group pattern. The between-group difference in hysteresis was, therefore, not attributable to the sex imbalance, although competitive level, sport discipline, and sex remain formally entangled in this design (Section 4.5).
Table 5.
Leg-spring hysteresis at the 0.42 m drop height stratified by group and sex.
To formally evaluate whether the sex imbalance between groups (international: 10 M/5 F; club: 10 M/15 F) accounted for the observed hysteresis differences, a two-way factorial ANOVA (general linear model) with group and sex as between-subjects fixed factors and their interaction was conducted. The group main effect on hysteresis remained large and highly significant in all three conditions after sex was entered into the model (BLJ: F(1,36) = 25.43, p < 0.001, η2p = 0.414; DOM: F(1,36) = 22.38, p < 0.001, η2p = 0.383; NDOM: F(1,36) = 30.05, p < 0.001, η2p = 0.455). A significant sex main effect was present for unilateral conditions (DOM: F(1,36) = 4.75, p = 0.036, η2p = 0.117; NDOM: F(1,36) = 6.98, p = 0.012, η2p = 0.162), with males exhibiting more negative hysteresis than females net of group, consistent with known sex differences in musculotendinous stiffness. Critically, no group × sex interaction reached significance in any condition (all p ≥ 0.27), indicating that the magnitude of the group difference was statistically homogeneous across sexes. Within the sex-balanced male stratum (n = 10 per group), between-group hysteresis differences remained large and significant across all conditions (BLJ d = −1.52, p = 0.003; DOM d = −1.37, p = 0.007; NDOM d = −1.77, p < 0.001). Collectively, these analyses indicate that the observed group differences in hysteresis were not attributable to the unequal sex composition of the two groups. These condition-specific models test the group contrast at the 0.42 m drop height; in the omnibus mixed-effects models in Section 3.5, the corresponding group term estimates the contrast at the 0.26 m reference level and is, therefore, not directly comparable with the values reported here (Table 6 and Table 7).
Table 6.
Linear mixed-effects model results for leg-spring hysteresis, adjusted for age and sex.
Table 7.
Linear mixed-effects model results for jump height, adjusted for age and sex.
3.4. Prevalence of Negative Hysteresis as a Whole-Limb Mechanical Pattern
At 0.26 m, the prevalence of negative hysteresis (reflecting net active energy contribution during concentric phase) was high in both groups across all conditions (international-level: 60–100%; club-level: 80–92%), with no statistically significant between-group difference (all Fisher’s exact tests p > 0.05; see Section 2.4 and Figure 2). At 0.42 m, international-level athletes maintained near-universal negative hysteresis (i.e., net active energy contribution) in the bilateral condition (100%), with 87% and 73% prevalence in the dominant and non-dominant unilateral conditions, respectively. In contrast, negative-hysteresis prevalence in club-level athletes collapsed substantially at 0.42 m (BLJ: 64%; DOM: 20%; NDOM: 12%), indicating that 80–88% of club-level athletes did not show negative whole-limb hysteresis under unilateral high-load conditions.
Figure 2.
Prevalence of negative hysteresis (proportion of athletes exhibiting net active energy contribution) across group and condition. BLJ = bilateral drop jump; DOM = dominant-leg drop jump; NDOM = non-dominant-leg drop jump. Black bars = international-level; grey bars = club-level. (A) 0.26 m drop height; (B) 0.42 m drop height. Comparisons at 0.26 m were non-significant.
The between-group difference in negative hysteresis prevalence was evaluated with Fisher’s exact test for each condition. At the 0.42 m drop height, the proportion of athletes exhibiting negative hysteresis was significantly greater in the international-level than in the club-level group in all three conditions: bilateral (15/15 vs. 16/25; p = 0.015), dominant-leg (13/15 vs. 5/25; p < 0.001), and non-dominant-leg (11/15 vs. 3/25; p < 0.001). At the 0.26 m drop height, the groups did not differ in any condition (all p > 0.05). These categorical results corroborate the continuous between-group hysteresis differences reported in Section 3.2.
3.5. Group × Drop-Height Interaction: Hysteresis and Jump Height
To examine whether age or sex accounted for the observed effects, age (covariate) and sex (fixed factor) were integrated into the linear mixed-effects models (LMMs). These adjusted models are reported below alongside the unadjusted estimates so that the influence of the demographic covariates on the group × drop-height interaction can be evaluated directly. Fixed effects were evaluated using Type III Wald chi-square tests (χ2). Categorical predictors were dummy-coded: group (0 = club, 1 = intl), sex (0 = female, 1 = male), drop height (0 = 0.26 m, 1 = 0.42 m). The reference condition was bilateral jump (BLJ).
A linear mixed-effects model (participant as a random intercept; group, drop height, condition, and their interactions as fixed effects) served as the primary omnibus analysis, accounting for the dependency across the repeated bilateral and unilateral conditions. For hysteresis, the group × drop-height interaction was very large (χ2(1) = 124.96, p < 0.001), with significant main effects of drop height (χ2(1) = 22.39, p < 0.001) and condition (χ2(2) = 38.25, p < 0.001); the group main effect was marginal (χ2(1) = 3.56, p = 0.059) and the group × condition, drop-height × condition, and three-way interactions were non-significant (all p ≥ 0.14). Because these are omnibus Type III tests, the direction of each effect is conveyed by the estimated marginal means reported below and by the signed, dummy-coded coefficients of the adjusted model in Table 6, rather than by standardized estimates. The LMM for hysteresis explained a substantial proportion of variance, yielding a marginal R2 (variance explained by fixed effects) of 0.48 and a conditional R2 (fixed plus random effects) of 0.76. The non-significant three-way interaction indicates that the group × drop-height crossover was statistically homogeneous across bilateral and unilateral conditions. Estimated marginal means reproduced the crossover: hysteresis in international-level athletes became more negative from 0.26 m to 0.42 m (−17.7% to −35.4%), whereas club-level athletes shifted from negative to net-dissipative (−29.7% to +14.0%). The corresponding individual-level trajectories for both dependent variables are displayed in Figure 3. After chronological age and sex were entered into the model, the group × drop-height interaction for leg-spring hysteresis remained highly significant and essentially unchanged relative to the unadjusted estimate (χ2(1) = 118.45, p < 0.001, B = −48.12 ± 4.42, βstd = −1.185), as did the main effect of drop height (χ2(1) = 35.30, p < 0.001, βstd = +0.838). Age was not a significant predictor of hysteresis (χ2(1) = 0.06, p = 0.799, βstd = −0.007), whereas sex contributed independently (χ2(1) = 12.48, p < 0.001, βstd = −0.359), males exhibiting more negative hysteresis than females net of competitive level. The group main effect was not significant in the adjusted model (χ2(1) = 0.00, p = 0.971). This estimate must be read in the light of the model parameterization: in the presence of a group × drop-height interaction, the group term is the between-group contrast at the reference level of drop height (0.26 m), at which no between-group difference in hysteresis was observed (Section 3.2). It, therefore, does not contradict the condition-specific analyses of Section 3.3, in which group was tested at 0.42 m and remained highly significant once sex had been entered; in the mixed-effects model, the caliber effect is carried entirely by the interaction term, consistent with a divergence expressed only under the more demanding eccentric load rather than as a constant group offset. The adjusted fixed-effects estimates are presented in Table 6.
Figure 3.
Individual-level trajectories for leg-spring hysteresis and jump height from the 0.26 m drop height to the 0.42 m drop height. Group means with 95% confidence intervals are overlaid on individual data lines. (A) Bilateral (BLJ) hysteresis; (B) bilateral (BLJ) jump height; (C) dominant-leg (DOM) hysteresis; (D) dominant-leg (DOM) jump height; (E) non-dominant-leg (NDOM) hysteresis; (F) non-dominant-leg (NDOM) jump height. Filled circles and solid lines = international-level; open squares and dashed lines = club-level.
For jump height, the model showed a large condition effect (χ2(2) = 2104.3, p < 0.001), a group effect (χ2(1) = 18.61, p < 0.001), a group × condition interaction (χ2(2) = 31.85, p < 0.001), and smaller group × drop-height (χ2(1) = 4.03, p = 0.045) and three-way (χ2(2) = 8.54, p = 0.014) interactions; as above, the direction of these effects is given by the estimated marginal means and by the signed coefficients of the adjusted model in Table 7. The jump height LMM demonstrated excellent explanatory power, with a marginal R2 of 0.52 and a conditional R2 of 0.88. In the age- and sex-adjusted model, athletic caliber remained the dominant predictor of jump height (χ2(1) = 75.10, p < 0.001, B = 0.1039 ± 0.0160, βstd = +1.194), together with sex (χ2(1) = 30.80, p < 0.001, βstd = +0.482) and drop height (χ2(1) = 14.60, p < 0.001, βstd = +0.272); the group × drop-height interaction also remained significant (χ2(1) = 11.95, p < 0.001, βstd = −0.402), whereas age was again non-significant (χ2(1) = 0.44, p = 0.507). The larger chi-square for this interaction relative to the unadjusted model reflects the omission of the higher-order condition interactions from the adjusted specification, which returns to the two-way term variance that the unadjusted model had partitioned into the three-way interaction. The adjusted fixed-effects estimates are presented in Table 7.
As descriptive decompositions of the omnibus mixed-effects models reported above, condition-specific 2 × 2 (group × drop height) mixed-design ANOVAs were additionally computed. Significant group × drop-height interactions were observed for hysteresis in all three conditions: BLJ (F(1,38) = 69.64, p < 0.001, η2p = 0.647), DOM (F(1,38) = 39.12, p < 0.001, η2p = 0.507), and NDOM (F(1,38) = 33.23, p < 0.001, η2p = 0.466). These represent very large interaction effects [22], indicating that the groups responded to increasing drop height with qualitatively opposite hysteresis trajectories. For jump height, a significant group × drop-height interaction was observed only in the bilateral condition (F(1,38) = 14.48, p < 0.001, η2p = 0.276). Unilateral jump height was statistically invariant across drop heights in both groups (DOM: F(1,38) = 0.21, p = 0.647; NDOM: F(1,38) = 0.07, p = 0.788). Full results are presented in Table 8.
Table 8.
Condition-specific 2 × 2 mixed-design ANOVAs used as descriptive decompositions of the interaction effects.
3.6. Regression Analysis: Prediction of Jump Height from Hysteresis
The regression models are presented in Table 9, and scatterplots are shown in Figure 4. Because the sample spanned the full caliber spectrum, these models were fitted to the pooled cohort (n = 40) and, therefore, describe the hysteresis–jump-height relationship across, rather than within, performance levels. Fitted to the pooled sample, hysteresis was a significant predictor of jump height in all three conditions at 0.42 m: BLJ (β = −0.714, R2 = 0.510, F(1,38) = 39.50, p < 0.001), DOM (β = −0.688, R2 = 0.474, F(1,38) = 34.18, p < 0.001), and NDOM (β = −0.661, R2 = 0.437, F(1,38) = 29.48, p < 0.001). The addition of a quadratic hysteresis term significantly improved model fit in the bilateral condition (ΔR2 = 0.092, ΔF(1,37) = 8.52, p = 0.006; total R2 = 0.601), and the inclusion of leg-spring stiffness as a second predictor yielded R2 = 0.560, with stiffness contributing a small but significant independent effect (β= 0.225, p = 0.046); both refinements were likewise estimated on the pooled sample. Within-group correlations, which isolate the association within a homogeneous caliber stratum, were more modest and condition-dependent (Table 10). In the international-level group, the relationship was strong for bilateral jumps (r = −0.772, p < 0.01) but did not reach significance in the non-dominant unilateral condition (r = −0.505, p > 0.05); in the club-level group, the bilateral correlation was non-significant (r = −0.373, p = 0.066), whereas the dominant and non-dominant correlations were moderate and significant (r = −0.562 and −0.518, respectively, both p < 0.01). Across the six group × condition cells, the within-stratum coefficients corresponded to 14–60% of explained variance, consistently at or below the pooled estimates, indicating that the larger pooled R2 values partly reflect the between-group separation in both hysteresis and jump height rather than a uniformly strong within-athlete dependency.
Table 9.
Regression models predicting jump height from leg-spring hysteresis at the 0.42 m drop height (n = 40).
Figure 4.
Association between leg-spring hysteresis and jump height at the 0.42 m drop height, by competitive level, for the (a) bilateral (BLJ), (b) dominant-leg (DOM), and (c) non-dominant-leg (NDOM) drop-jump conditions. International-level athletes are shown as filled circles with a solid group-specific regression line; club-level athletes are shown as open squares with a dashed group-specific regression line (international-level, n = 15; club-level, n = 25). The light-grey solid line is the full-sample linear fit; in panel (a), the grey dotted curve is the full-sample quadratic fit. Inset values in panel (a) are within-group Pearson correlations (intl, club) and pooled coefficients of determination for the linear (R2) and quadratic (quad R2) models. Negative hysteresis denotes a net active energy contribution (negative whole-limb hysteresis pattern); positive hysteresis denotes net dissipation. Within each group, more negative hysteresis was associated with greater jump height across all three conditions, and the international-level group occupied the more negative region of every panel.
Table 10.
Within-group Pearson correlations between leg-spring hysteresis and jump height at the 0.42 m drop height.
To determine whether these pooled associations reflected a within-level relationship or the separation between cohorts, each 0.42 m regression was re-estimated with group as a covariate and with a group × hysteresis interaction term (Table 11). Hysteresis remained a significant predictor of jump height after adjustment for group in all three conditions (all p ≤ 0.001), contributing incremental variance beyond group of ΔR2 = 0.26 (BLJ), 0.20 (DOM), and 0.20 (NDOM). Because group alone explained R2 = 0.25–0.28 relative to the pooled R2 = 0.44–0.51, approximately half of the pooled explanatory power was attributable to between-group separation. A group × hysteresis interaction was significant only for the bilateral condition (p = 0.029): the hysteresis–jump-height slope was steep within international-level athletes (r = −0.77, p < 0.001) but weak and non-significant within club-level athletes (r = −0.37, p = 0.066). For the unilateral conditions, the slopes were parallel across groups and both moderate (DOM: international r = −0.54, club r = −0.56; NDOM: international r = −0.50, club r = −0.52). The pooled models, therefore, describe an association that is partly driven by caliber separation and, for bilateral jumping, is expressed most strongly within the international-level cohort; the within-level relationship is moderate and condition-dependent.
Table 11.
Group-adjusted regression of 0.42 m jump height on leg-spring hysteresis, by condition.
3.7. Methodological Sensitivity Analysis (CoM vs. HJC Models)
To demonstrate that our correlations and group differences are stable and not sensitive to methodological alterations, we re-analyzed the relationship between jump height and hysteresis in the two unilateral conditions using both the primary hip-joint-center (HJC) tracking model defined in Section 2.4 and an alternative whole-body center-of-mass (CoM) tracking model, at the demanding 0.42 m drop height.
Under the dominant-leg condition (DOM at 0.42 m), the correlation between jump height and hysteresis remained highly consistent, yielding r = −0.688 (p < 0.01) for the primary HJC-derived model and r = −0.654 (p < 0.01) for the alternative CoM-derived model. Similarly, under the non-dominant-leg condition (NDOM at 0.42 m), the HJC-derived correlation (r = −0.661, p < 0.01) was closely mirrored by the CoM-derived model (r = −0.632, p < 0.01).
Furthermore, the significant group × drop-height interaction effects for hysteresis remained highly robust regardless of the tracking model used (all p < 0.001), as did the between-group contrasts at 0.42 m (all |d| > 1.50). In both tracking configurations, international-level athletes consistently exhibited highly negative hysteresis (net active energy contribution), whereas club-level athletes shifted to net positive/dissipative values at 0.42 m. This methodological comparison indicates that the observed associations and group separations were robust to the choice of tracking model.
3.8. Trial Selection Sensitivity Analysis (Best Trial vs. Mean of Three Trials)
Because the primary analyses retained the single highest-jump trial per condition, and because jump height is itself a dependent variable subsequently associated with hysteresis, all 0.42 m models were re-estimated using the mean of each participant’s three valid trials to verify that the reported hysteresis–jump-height relationships were not an artefact of maximal-trial selection. Averaging across trials left the group means essentially unchanged while narrowing the standard deviations by approximately 4–7%, consistent with the expected reduction in measurement error. At 0.42 m, mean-of-three hysteresis values were −47.2 ± 29.8% (BLJ), −26.9 ± 23.1% (DOM), and −26.5 ± 30.2% (NDOM) in the international-level group, and +1.2 ± 24.1%, +20.1 ± 28.5%, and +18.4 ± 17.2%, respectively, in the club-level group, closely mirroring the best-trial values reported in Table 3 and preserving the direction and magnitude of the between-group separation.
The linear regression of jump height on hysteresis was likewise stable, with the explained variance marginally higher than in the best-trial models: BLJ (β = −0.736, R2 = 0.542, adjusted R2 = 0.530, B = −0.00124, p < 0.001), DOM (β = −0.713, R2 = 0.508, adjusted R2 = 0.495, B = −0.00092, p < 0.001), and NDOM (β = −0.682, R2 = 0.465, adjusted R2 = 0.451, B = −0.00091, p < 0.001) (see Table 12). The slightly larger coefficients of determination relative to the best-trial models (Table 9; R2 = 0.437–0.510) indicate that the hysteresis–jump-height association reflects a stable mechanical characteristic of the athlete rather than a dependence on extreme single-trial performances. Critically, when group was entered first in a hierarchical model, hysteresis retained a significant incremental contribution to jump height under the mean-of-three specification (ΔR2 = 0.274 [BLJ], 0.218 [DOM], and 0.205 [NDOM], all p < 0.001), paralleling the group-adjusted best-trial results (Table 11; ΔR2 = 0.197–0.260). The best-trial and mean-of-three analyses, therefore, converge, indicating that the trial selection strategy did not materially influence the reported associations.
Table 12.
Regression models predicting jump height from leg-spring hysteresis at the 0.42 m drop height using the mean of three trials (n = 40).
4. Discussion
This study examined leg-spring hysteresis and jump height in international-level track-and-field athletes and club-level multi-sport athletes across bilateral and unilateral drop-jump conditions from two drop heights. Three principal findings were obtained. First, the two groups responded to increasing drop heights with qualitatively opposite hysteresis trajectories. Second, these divergent adaptations were reflected in very large group × drop-height interaction effects for hysteresis (η2p = 0.466–0.647), without corresponding interactions for unilateral jump height. Third, hysteresis was a significant predictor of jump height, in the pooled sample, at 0.42 m (R2 = 0.44–0.60), with the bilateral condition exhibiting a unique curvilinear relationship.
4.1. Differential Hysteresis Responses as a Whole-Limb Mechanical Marker
The divergent hysteresis trajectories align with the theoretical expectation that international-level athletes possess superior musculotendinous stiffness regulation capacities, allowing them to exploit increased eccentric loading at the 0.42 m drop height [10,11,26]. This divergence is quantified in the between-group comparison (Table 3): whereas the two groups were statistically indistinguishable in hysteresis at 0.26 m, at 0.42 m, the international-level athletes became markedly more negative, while the club-level athletes shifted toward net energy dissipation. Because elite athletic level in this study was co-aligned with a specialized track-and-field training background, this response likely reflects a collective neuromuscular phenotype optimized for explosive, elastic-recoil tasks, rather than competitive caliber in isolation [14,19]. The 100% negative hysteresis prevalence in international-level athletes during bilateral jumps and the near-complete collapse in club-level athletes at 0.42 m (Figure 2; 12–64% depending on condition), together with the individual trajectories in Figure 3 that show the separation was not driven by a small number of outliers, are consistent with international-level athletes possessing neuromuscular and musculotendinous stiffness profiles that better preserve a negative whole-limb hysteresis pattern under increasing drop height. Because competitive level was confounded with sex, we verified that this pattern was not an artefact of the sex imbalance: the sex-stratified descriptives (Table 5) show that the group difference in 0.42 m hysteresis persisted within the sex-balanced male stratum, indicating a caliber-related rather than a purely sex-related effect. This interpretation is consistent with longitudinal evidence that plyometric training reduces tendon hysteresis during ballistic contractions [9] and with cross-sectional evidence that elite athletes display a sport-specific capacity to use elastic energy in the patellar and Achilles tendons [27], extending that evidence base from the isolated tendon to the whole-limb spring. We explicitly acknowledge that leg-spring hysteresis is a global, whole-limb mechanical quantity derived from the force–length loop, rather than a direct measurement of localized tendon or muscle behavior; therefore, any tendon-level interpretations in this cohort remain inferential.
The neuromechanical basis for this international-level advantage likely operates through multiple interdependent pathways. First, the temporal precision of pre-activation is critical: activation of the plantar flexors, quadriceps, and hip extensors before ground contact stiffens the musculotendinous unit prior to impact [28,29]. Second, direct ultrasonographic evidence has established that, in trained athletes, the gastrocnemius fascicles maintain a relatively isometric length during the braking phase while the Achilles tendon undergoes predominant elongation, a functional decoupling termed the catapult mechanism [30,31]. Third, the rapidly increasing eccentric loading rate at impact triggers a short-latency myotatic reflex response whose potentiation in trained athletes augments force production during the early concentric phase [29]. Structural adaptation through chronic loading is further evidenced by low-hysteresis tendons in trained athletes that transfer a greater proportion of stored energy into the propulsive phase [9,27].
4.2. Interaction Effects and the Role of Drop Height as a Diagnostic Load
The absence of a significant group × drop-height interaction for unilateral jump height, despite highly significant interactions for hysteresis under the same conditions (Table 8), represents an important mechanistic dissociation. The between-group jump-height comparison (Table 4) shows that international-level athletes jumped higher in every condition at both drop heights (d = 1.14–1.77), yet the mixed-model interaction reveals that they achieved this superiority through qualitatively different, drop-height-dependent mechanical strategies that scalar jump height alone does not capture. The individual trajectories in Figure 3 make this explicit: the two groups moved in opposite hysteresis directions as drop height increased, even though both preserved their jump-height ranking. The 0.26 m condition was insufficient to reveal between-group differences in whole-limb energy management, as the mechanical stimulus did not exceed the adaptive capacity of club-level athletes; the 0.42 m condition, therefore, appeared, within the present sample and protocol, to be a more diagnostically sensitive loading condition, particularly in unilateral contexts. It is worth noting that this crossover was bidirectional rather than a divergence from a common baseline. At 0.26 m, the club-level athletes were in fact numerically more negative than the international-level athletes in both unilateral conditions (DOM, −33.97% versus −8.96%; NDOM, −21.57% versus −9.85%; Table 3), and their dispersion at this drop height was two- to three-times larger (SD = 44–61% versus 23–26%). Under a low eccentric load, the club-level group, therefore, appears to have been mechanically heterogeneous, with individual athletes adopting markedly different force–length loop strategies, whereas the higher load elicited a more uniform and predominantly dissipative response. The contraction of within-group variability from 0.26 m to 0.42 m in this cohort is itself informative, indicating that the diagnostic value of the higher drop height lies not only in separating the group means but in narrowing the range of mechanical solutions that remain viable under load.
These findings are consistent with and extend prior investigations of stiffness and performance across skill levels. Laffaye et al. [16] compared expert jumpers drawn from several sports with novice participants during a maximal run-and-jump task and found no difference in leg-spring stiffness between expertise levels. The present study offers a mechanical account of that null result by demonstrating that stiffness alone—without concurrent evaluation of the force–length loop area—can obscure a mechanically fundamental distinction: two athletes may display comparable stiffness magnitudes yet differ radically in their capacity to recover stored elastic energy, as indexed by the sign and magnitude of hysteresis. The absence of between-group hysteresis differences at 0.26 m (Table 3), despite substantial jump-height differences at the same height (Table 4; Cohen’s d = 1.14–1.77), parallels observations by Healy et al. [15] that drop heights must be sufficiently demanding to unmask inter-individual differences in reactive-jumping capacity. The 0.42 m condition used here corresponds to a gravitational potential energy approximately 62% greater than the 0.26 m condition, and the resulting eccentric loading impulse appears to exceed the adaptive capacity of club-level musculotendinous systems, unmasking the divergence in hysteresis trajectories [4,11,32].
4.3. Hysteresis as a Predictor of Jump Performance
The pooled associations between hysteresis and jump height (Table 9; R2 = 0.44–0.60) indicate that whole-limb force–length loop behavior is mechanically relevant to vertical jump performance across the caliber spectrum sampled here, consistent with reports that reactive-strength qualities are associated with independent markers of athletic performance [17]. This pooled estimate should, however, be read with two constraints. First, because performance level separated both hysteresis and jump height, the pooled coefficients incorporate between-group (caliber) variance; the within-stratum associations (Table 10) were more modest and condition-dependent (|r| = 0.37–0.77; 14–60% of variance), and the group-adjusted models (Table 11) show that hysteresis retained only ΔR2 ≈ 0.20–0.26 once group was partialled out, with a significant group × hysteresis interaction in the bilateral condition alone. The relationship is, therefore, better characterized as moderate within a given caliber level and amplified when athletes spanning the performance range are pooled, a pattern visible in the group-specific regression lines in Figure 4. Second, hysteresis and jump height were both derived from the kinematics and kinetics of the same trials, so the association is partly one of shared mechanical origin rather than prediction of an independent outcome, and the present cross-sectional design cannot establish that altering hysteresis would change jump height. The strongly negative individual values observed in some international-level athletes (approaching −80 to −95%) should, therefore, be read as evidence of substantial net concentric contribution during propulsion rather than as implausibly large elastic recoil: a passive spring cannot return more energy than it stores, so negative whole-limb hysteresis necessarily reflects active power generation [33]. This reinforces our interpretation of leg-spring hysteresis as a whole-limb mechanical descriptor rather than a tendon-level elasticity index. That both measures were highly reliable within session (Table 2) makes measurement error an unlikely source of these associations. With these caveats, the unstandardized slopes (Table 9; B ≈ −0.00094 to −0.00127) translate to approximately a 0.9–1.3 mm change in jump height per percentage-point change in hysteresis. The curvilinear improvement in the bilateral model (ΔR2 = 0.092, p = 0.006) and the small but significant stiffness contribution (β = 0.225, p = 0.046), both estimated on the pooled sample, suggest a nonlinear bilateral force–length relationship and confirm that stiffness and hysteresis capture partially distinct variance.
4.4. Bilateral–Unilateral Asymmetry in Hysteresis
The bilateral condition exhibited substantially larger η2p values for both the group × drop-height interaction (η2p = 0.647) and the jump-height interaction (η2p = 0.276) than the unilateral conditions (Table 8). Under bilateral loading, the total eccentric impulse is shared between both lower extremities, effectively halving the per-limb mechanical demand relative to the unilateral case [34]. This load-sharing configuration likely provides a more favorable mechanical environment for a negative whole-limb hysteresis pattern, explaining why even club-level athletes maintained a relatively higher negative hysteresis prevalence in bilateral conditions at 0.42 m (Figure 2; 64%) compared with the near-complete collapse under unilateral high-load conditions (DOM: 20%; NDOM: 12%). The dissociation between the significant bilateral jump-height interaction and the absence of significant unilateral jump-height interactions, despite highly significant unilateral hysteresis interactions (Table 8), reveals that scalar performance metrics can be preserved through compensatory joint-level strategies even when the global whole-limb force–length loop behavior is altered [5]. International-level athletes appear to achieve superior unilateral jump height via a mechanically distinct active mechanical strategy, whereas club-level athletes at high unilateral loads may rely more heavily on rate-of-force development and impulse duration. This pattern is tentatively consistent with the bilateral deficit phenomenon documented in power athletes [35], although the mechanistic relevance of this concept to reactive-jumping hysteresis requires direct empirical verification.
4.5. Limitations
The principal limitation is that athletic caliber was structurally confounded with both sport discipline and sex. The international-level group consisted exclusively of track-and-field athletes, whereas the club-level group was predominantly composed of ball-sport athletes (only 2 of 25 were track-and-field competitors); the groups also differed in sex composition (Table 1; 10 M/5 F versus 10 M/15 F). Consequently, the observed differences should be interpreted as a multi-factorial neuromuscular phenotype of highly trained elastic-recoil specialists rather than being attributed to performance caliber per se. While the group differences persisted strongly within the sex-balanced male stratum (confirming the robust nature of the trend), future investigations employing sex-matched and discipline-matched cohorts are warranted to isolate the independent contributions of athletic caliber from sport-specific mechanical adaptations. Two observations bound this ambiguity without resolving it: the negative-hysteresis signature was present across mechanically dissimilar track-and-field disciplines within the elite group (Section 3.3), and the group effect was robust to adjustment for the one confounder that did vary within groups, namely chronological age. Definitive separation of caliber, discipline, and sex requires replication in discipline-matched and sex-balanced cohorts. Additional limitations include the constrained and unequal sample size (n = 40; 15 versus 25), the forefoot-landing instruction that constrains natural foot-strike patterns, the bilateral midpoint HJC approximation that assumes symmetrical limb loading, and the use of absolute rather than stature- or leg-length-normalized drop heights. Because the eccentric loading imposed at touchdown scales with the potential energy of the drop, a fixed absolute height represents a different relative mechanical demand for a taller than for a shorter athlete, and the groups were not matched on the segment lengths that govern this scaling; part of the divergence at 0.42 m may, therefore, reflect differences in relative rather than absolute loading intensity, and future work should normalize drop height to leg length or stature. Two further constraints follow from the trial selection and signal-processing choices. A mean-of-three-trials sensitivity analysis (Section 3.8) confirmed that the reported hysteresis–jump-height associations and group separations were robust to the choice of trial selection strategy, with group means and regression coefficients remaining essentially unchanged. While kinematics and kinetics were subjected to different filtering frequencies in the primary analysis, a comprehensive sensitivity analysis (comparing unfiltered GRF with several cutoff frequencies, including a matched 12 Hz filter) confirmed that this asymmetry did not distort the hysteresis calculations. The integrated nature of the force–length loop area renders it robust to high-frequency transients, and the use of zero-lag filters prevented any artificial phase-shift discrepancies.
4.6. Practical Implications
Under the present testing conditions, leg-spring hysteresis appeared to be a sensitive biomechanical marker for differentiating the reactive-jumping capacity of these two cohorts. Practitioners should consider incorporating multi-height bilateral and unilateral drop-jump assessments into performance profiling batteries, as a single 0.26 m drop height is insufficient to reveal the full spectrum of differences in whole-limb energy management. The finding that 80–88% of club-level athletes did not show negative whole-limb hysteresis under unilateral high-load conditions identifies whole-limb energy return patterning as a potentially relevant adaptive target. Future prospective training studies could investigate whether bilateral-to-unilateral plyometric progressions benefit from force–length loop monitoring, and whether negative whole-limb hysteresis during bilateral drop jumps from 0.42 m might serve as a hypothesis-driven threshold for advancing to unilateral high-shock plyometrics. Displaying force–length loops in real time could also serve as a potential biofeedback modality to optimize pre-activation timing, though this requires prospective validation.
5. Conclusions
This study demonstrated that international-level track-and-field athletes and club-level multi-sport athletes diverge in their leg-spring hysteresis responses to increasing drop heights: international-level athletes responded to elevated drop heights with progressively more negative hysteresis (a pattern consistent with greater active contribution during unloading), whereas club-level athletes responded with net mechanical energy dissipation at 0.42 m. These qualitatively distinct responses were captured by very large group × drop-height interactions for hysteresis across bilateral and unilateral conditions (η2p = 0.466–0.647) and were not apparent at 0.26 m, suggesting that a sufficiently demanding eccentric load may be required to unmask between-group differences in whole-limb energy management within the present sample. The near-universal prevalence of negative hysteresis in international-level athletes under bilateral loading (100%) and its collapse in the majority of club-level athletes under unilateral high-load conditions (DOM: 20%; NDOM: 12%) points to a single-limb, high-load condition, not apparent under bilateral testing, under which whole-limb force–length loop behavior differentiated the two cohorts. Notably, a significant group × drop-height interaction for jump height emerged only in the bilateral condition, indicating that scalar performance metrics may be preserved through compensatory mechanical strategies even when the whole-limb force–length loop behavior is altered. Pooled across the sampled caliber range, hysteresis accounted for 44–60% of the variance in jump height at 0.42 m, with leg-spring stiffness contributing small additional independent variance in the bilateral model; within a single caliber stratum, this association was more modest and condition-dependent. These findings suggest that the integration of multi-height, bilateral, and unilateral force–length loop analysis into biomechanical performance screening may offer meaningful diagnostic sensitivity beyond conventional jump-height metrics.
Supplementary Materials
The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/app16178449/s1, Figure S1: Individual leg-spring hysteresis values at the 0.42 m drop height for the (a) bilateral (BLJ), (b) dominant-leg (DOM) and (c) non-dominant-leg (NDOM) drop-jump conditions, disaggregated by competitive level, sex and sport discipline. Each marker is one athlete; marker colour denotes sport discipline and marker shape denotes sex (circles = male, triangles = female). Horizontal bars show the group × sex mean ± SD. The dashed line at 0% separates net dissipation (positive hysteresis, above the line) from a negative whole-limb hysteresis pattern indicating net active energy contribution (below the line). Intl = international-level track-and-field athletes; Club = club-level multi-sport athletes; M = male; F = female; T&F = track and field. The negative-hysteresis signature of the international-level group is present in both sexes and across mechanically dissimilar track-and-field disciplines, including the throwing subgroup. Table S1: Sensitivity Analysis: Leg-Spring Hysteresis (%) Under Different GRF Cutoff Frequencies at 0.42 m Drop Height, Bilateral Drop-Jump Condition (n = 40).
Author Contributions
Conceptualization, Ö.K., M.Y.K. and A.A.; methodology, Ö.K. and M.Y.K.; software, M.Y.K.; validation, Ö.K., M.Y.K. and B.K.; formal analysis, M.Y.K.; investigation, Ö.K. and B.K.; resources, Ö.K.; data curation, Ö.K.; writing—original draft preparation, Ö.K.; writing—review and editing, Ö.K., M.Y.K., B.K. and A.A.; visualization, A.A.; supervision, project administration, Ö.K. All authors have read and agreed to the published version of the manuscript.
Funding
This research received no external funding.
Institutional Review Board Statement
The study was conducted in accordance with the Declaration of Helsinki and approved by the Non-Interventional Clinical Research Ethics Committee (Approval No. 232; date: 30 November 2022).
Informed Consent Statement
Informed consent was obtained from all subjects involved in the study.
Data Availability Statement
The data presented in this study are available on request from the corresponding author. The data are not publicly available due to privacy restrictions.
Conflicts of Interest
The authors declare no conflicts of interest.
References
- Blickhan, R. The spring-mass model for running and hopping. J. Biomech. 1989, 22, 1217–1227. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- McMahon, T.A.; Cheng, G.C. The mechanics of running: How does stiffness couple with speed? J. Biomech. 1990, 23, 65–78. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Rogers, S.A.; Whatman, C.S.; Pearson, S.N.; Kilding, A.E. Assessments of mechanical stiffness and relationships to performance determinants in middle-distance runners. Int. J. Sports Physiol. Perform. 2017, 12, 1329–1334. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Arampatzis, A.; Brüggemann, G.-P.; Metzler, V. The effect of speed on leg stiffness and joint kinetics in human running. J. Biomech. 1999, 32, 1349–1353. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Maloney, S.J.; Fletcher, I.M. Lower limb stiffness testing in athletic performance: A critical review. Sports Biomech. 2021, 20, 109–130. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ker, R.F. Dynamic tensile properties of the plantaris tendon of sheep (Ovis aries). J. Exp. Biol. 1981, 93, 283–302. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- A Cavagna, G.; Dusman, B.; Margaria, R. Positive work done by a previously stretched muscle. J. Appl. Physiol. 1968, 24, 21–32. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Maganaris, C.N.; Paul, J.P. Tensile properties of the in vivo human gastrocnemius tendon. J. Biomech. 2002, 35, 1639–1646. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kubo, K.; Ikebukuro, T.; Yata, H. Effects of plyometric training on muscle–tendon mechanical properties and behavior of fascicles during jumping. Physiol. Rep. 2021, 9, e15073. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Arampatzis, A.; Schade, F.; Walsh, M.; Brüggemann, G.-P. Influence of leg stiffness and its effect on myodynamic jumping performance. J. Electromyogr. Kinesiol. 2001, 11, 355–364. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Struzik, A. Measuring Leg Stiffness During Vertical Jumps: Theory and Methods; Springer: Cham, Switzerland, 2019. [Google Scholar] [CrossRef] [Scilit]
- Komi, P.V. Physiological and biomechanical correlates of muscle function: Effects of muscle structure and stretch-shortening cycle on force and speed. Exerc. Sport Sci. Rev. 1984, 12, 81–122. [Google Scholar] [CrossRef] [Scilit]
- Bosco, C.; Komi, P.V. Potentiation of the mechanical behavior of the human skeletal muscle through prestretching. Acta Physiol. Scand. 1979, 106, 467–472. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kuitunen, S.; Komi, P.V.; Kyröläinen, H. Knee and ankle joint stiffness in sprint running. Med. Sci. Sports Exerc. 2002, 34, 166–173. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Healy, R.; Kenny, I.C.; Harrison, A.J.; Harrison, D. Reactive strength index: A poor indicator of reactive strength? Int. J. Sports Physiol. Perform. 2018, 13, 802–809. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Laffaye, G.; Bardy, B.G.; Durey, A. Leg stiffness and expertise in men jumping. Med. Sci. Sports Exerc. 2005, 37, 536–543. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jarvis, P.; Turner, A.; Read, P.; Bishop, C. Reactive strength index and its associations with measures of physical and sports performance: A systematic review with meta-analysis. Sports Med. 2021, 52, 301–330. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ramirez-Campillo, R.; Thapa, R.K.; Afonso, J.; Perez-Castilla, A.; Bishop, C.; Byrne, P.J.; Granacher, U. Effects of plyometric jump training on the reactive strength index in healthy individuals across the lifespan: A systematic review with meta-analysis. Sports Med. 2023, 53, 1029–1053. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Farris, D.J.; Sawicki, G.S. The mechanics and energetics of human walking and running: A joint level perspective. J. R. Soc. Interface 2011, 9, 110–118. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Urbaniak, G.C.; Plous, S. Research Randomizer (Version 4.0) [Computer Software]. Available online: https://www.randomizer.org/ (accessed on 17 June 2024).
- Bell, A.L.; Brand, R.A.; Pedersen, D.R. Prediction of hip joint centre location from external landmarks. Hum. Mov. Sci. 1989, 8, 3–16. [Google Scholar] [CrossRef] [Scilit]
- Cohen, J. Statistical Power Analysis for the Behavioral Sciences, 2nd ed.; Lawrence Erlbaum Associates: Hillsdale, NJ, USA, 1988. [Google Scholar] [CrossRef] [Scilit]
- Koo, T.K.; Li, M.Y. A guideline of selecting and reporting intraclass correlation coefficients for reliability research. J. Chiropr. Med. 2016, 15, 155–163. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Faul, F.; Erdfelder, E.; Lang, A.-G.; Buchner, A. G*Power 3: A flexible statistical power analysis program for the social, behavioral, and biomedical sciences. Behav. Res. Methods 2007, 39, 175–191. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Miller, G.A.; Chapman, J.P. Misunderstanding analysis of covariance. J. Abnorm. Psychol. 2001, 110, 40–48. [Google Scholar] [CrossRef] [PubMed]
- Komi, P.V. (Ed.) Strength and Power in Sport, 2nd ed.; Blackwell Publishing: Oxford, UK, 2003. [Google Scholar] [CrossRef] [Scilit]
- Wiesinger, H.-P.; Rieder, F.; Kösters, A.; Müller, E.; Seynnes, O.R. Sport-specific capacity to use elastic energy in the patellar and Achilles tendons of elite athletes. Front. Physiol. 2017, 8, 132. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gollhofer, A.; Strojnik, V.; Rapp, W.; Schweizer, L. Behaviour of triceps surae muscle-tendon complex in different jump conditions. Eur. J. Appl. Physiol. Occup. Physiol. 1992, 64, 283–291. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Avela, J.; Komi, P.V. Reduced stretch reflex sensitivity and muscle stiffness after long-lasting stretch-shortening cycle exercise in humans. Eur. J. Appl. Physiol. Occup. Physiol. 1998, 78, 403–410. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kurokawa, S.; Fukunaga, T.; Fukashiro, S. Behavior of fascicles and tendinous structures of human gastrocnemius during vertical jumping. J. Appl. Physiol. 2001, 90, 1349–1358. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kawakami, Y.; Muraoka, T.; Ito, S.; Kanehisa, H.; Fukunaga, T. In vivo muscle fibre behaviour during counter-movement exercise in humans reveals a significant role for tendon elasticity. J. Physiol. 2002, 540, 635–646. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wilson, G.J.; Wood, G.A.; Elliott, B.C. Optimal stiffness of series elastic component in a stretch-shorten cycle activity. J. Appl. Physiol. 1991, 70, 825–833. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zelik, K.E.; Franz, J.R. It’s positive to be negative: Achilles tendon work loops during human locomotion. PLoS ONE 2017, 12, e0179976. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Howard, J.D.; Enoka, R.M. Maximum bilateral contractions are modified by neurally mediated interlimb effects. J. Appl. Physiol. 1991, 70, 306–316. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pain, M.T. Considerations for single and double leg drop jumps: Bilateral deficit, standardizing drop height, and equalizing training load. J. Appl. Biomech. 2014, 30, 722–727. [Google Scholar] [CrossRef] [Scilit] [PubMed]
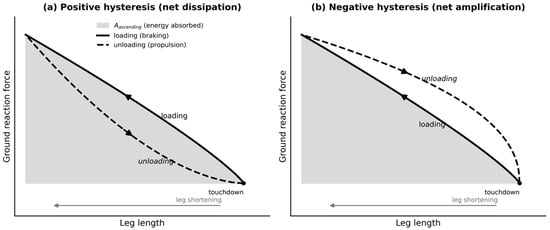
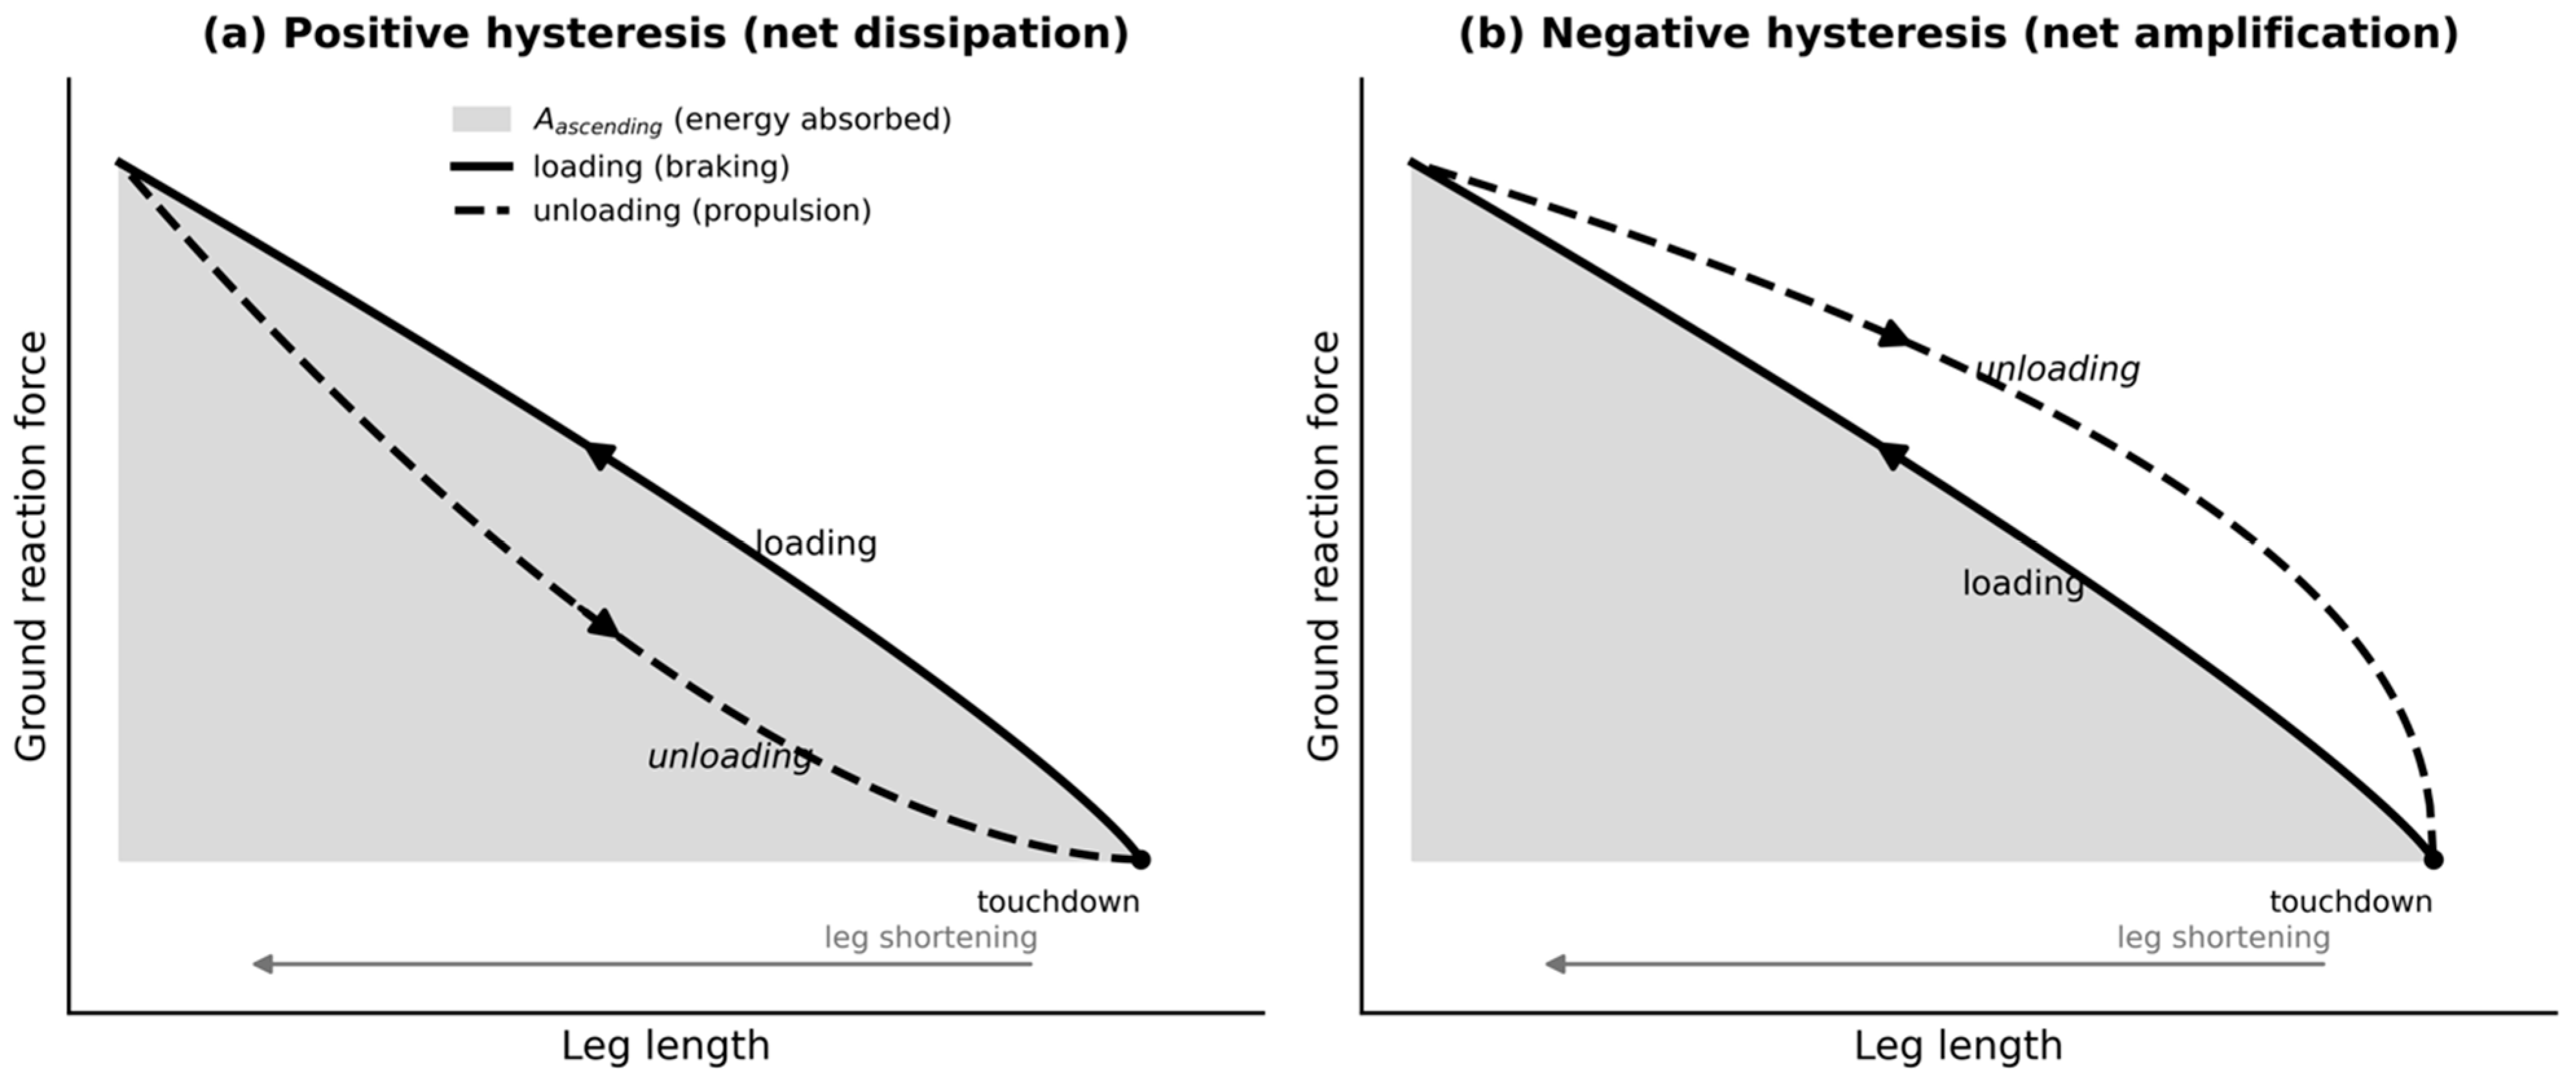
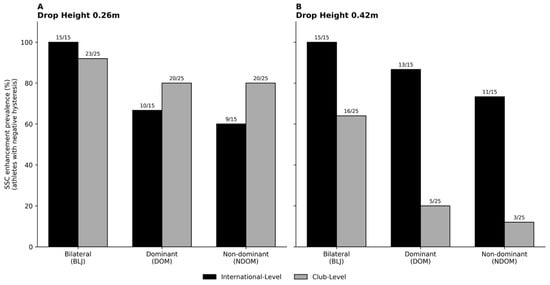
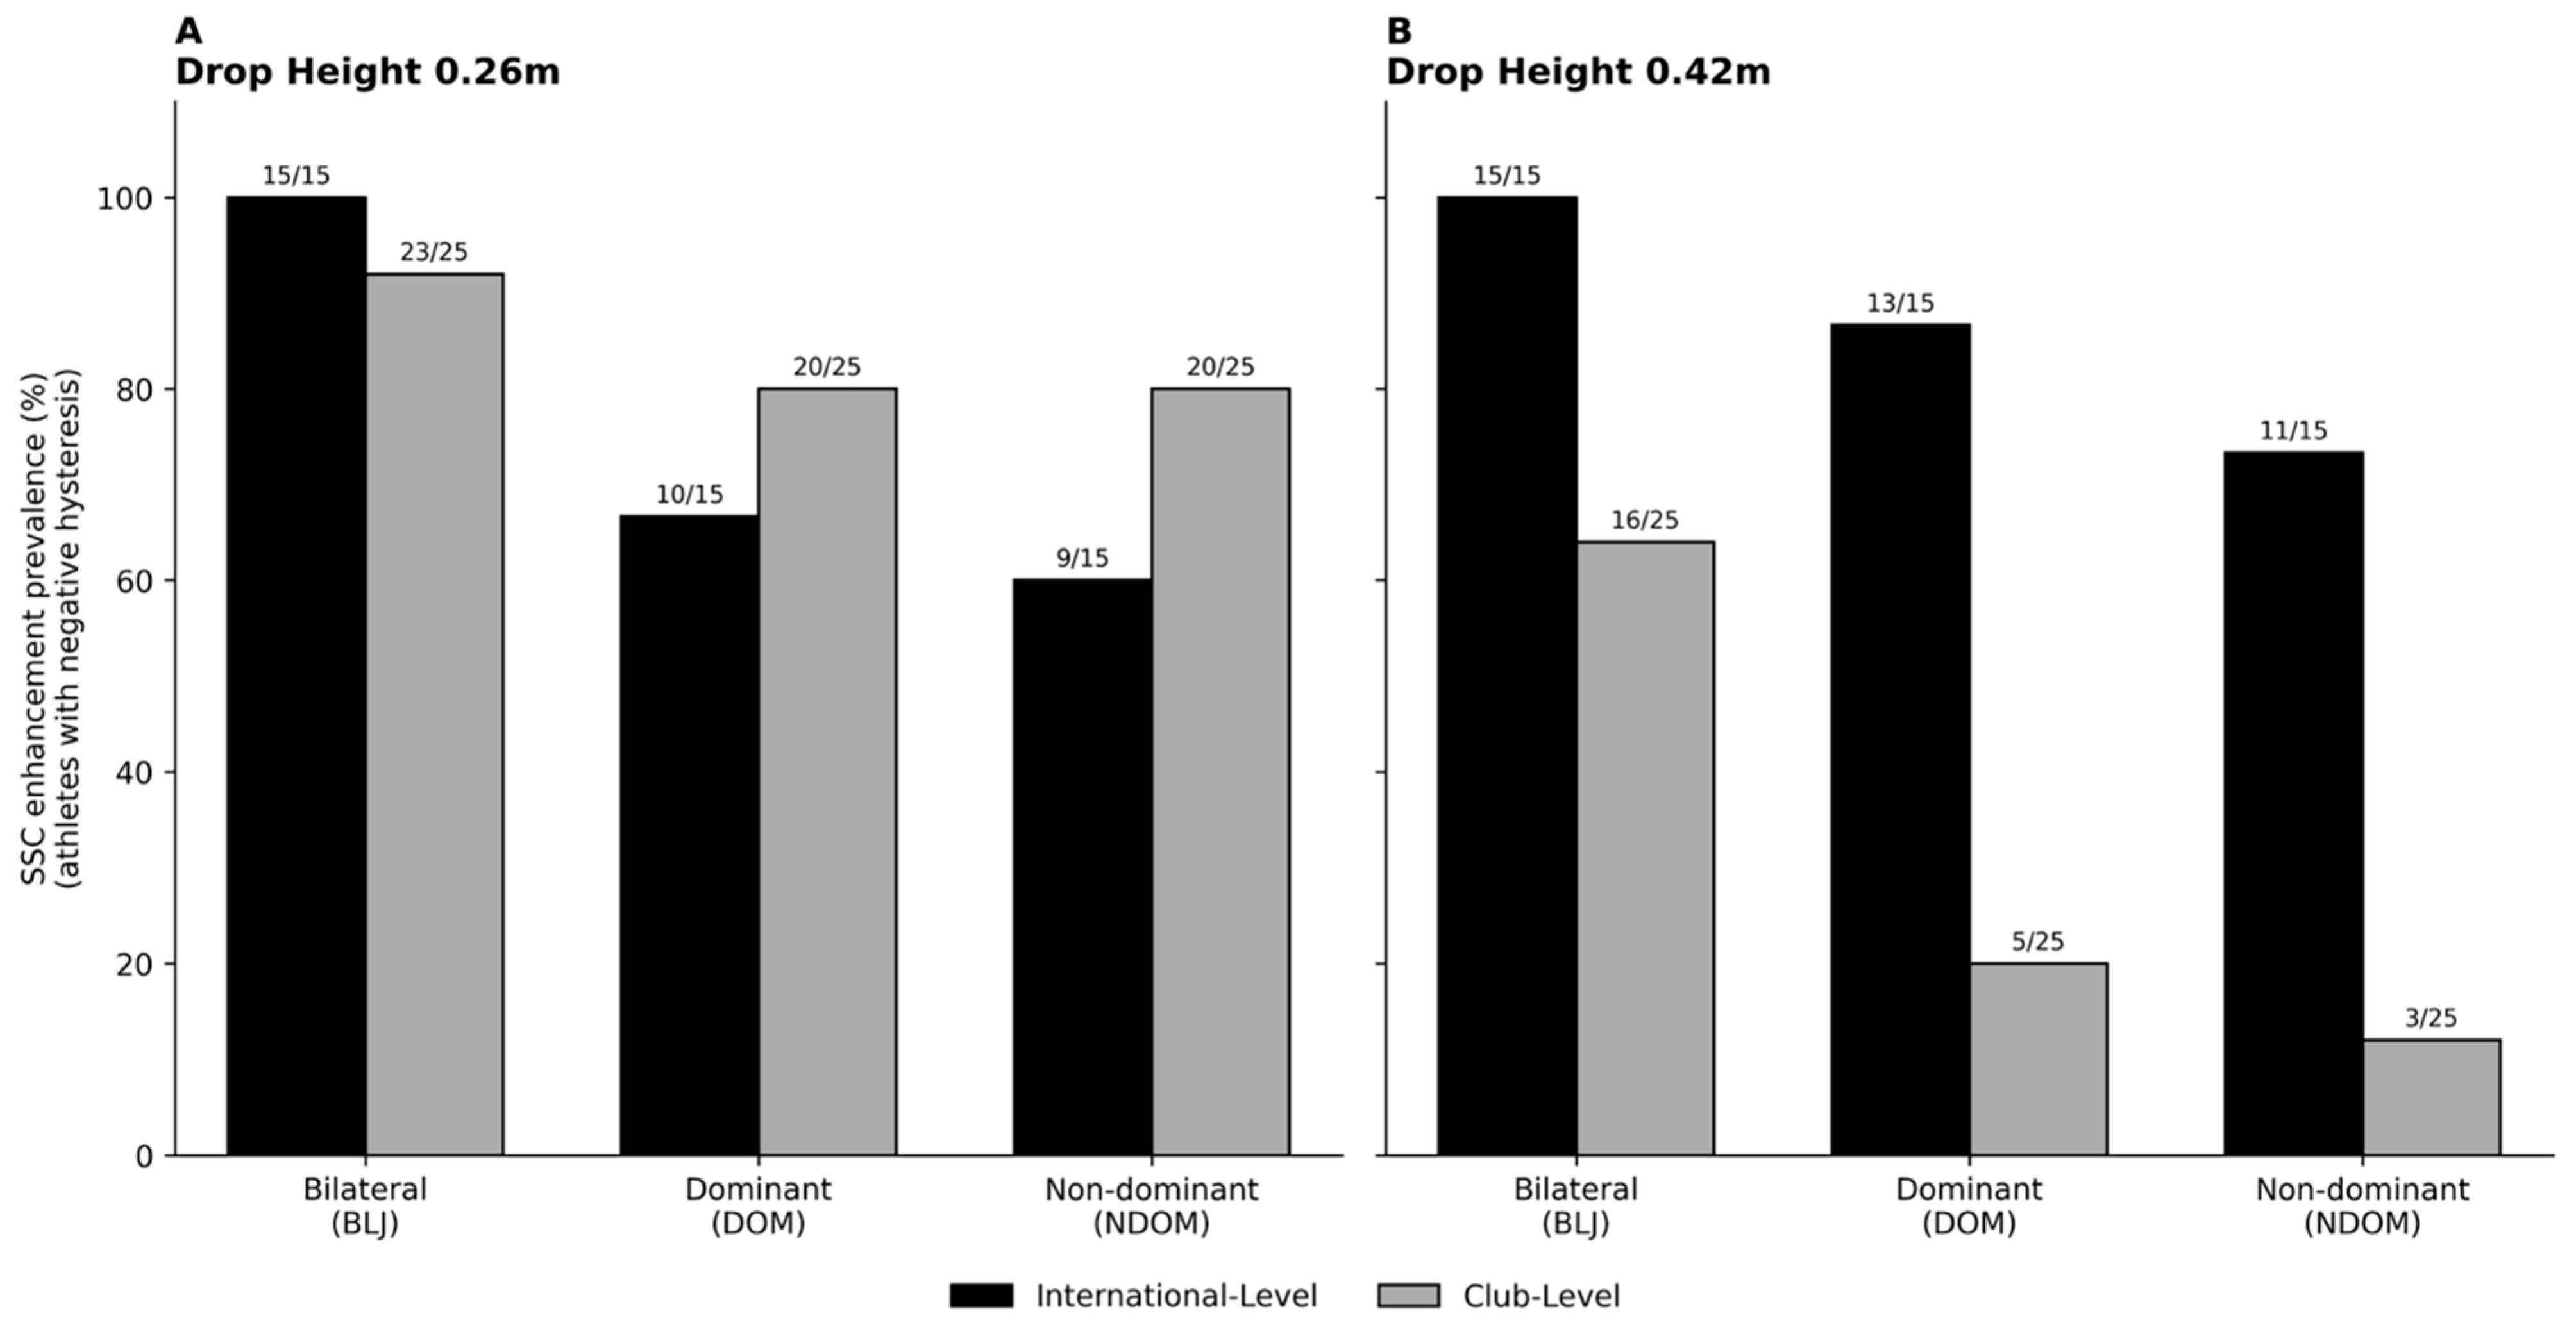
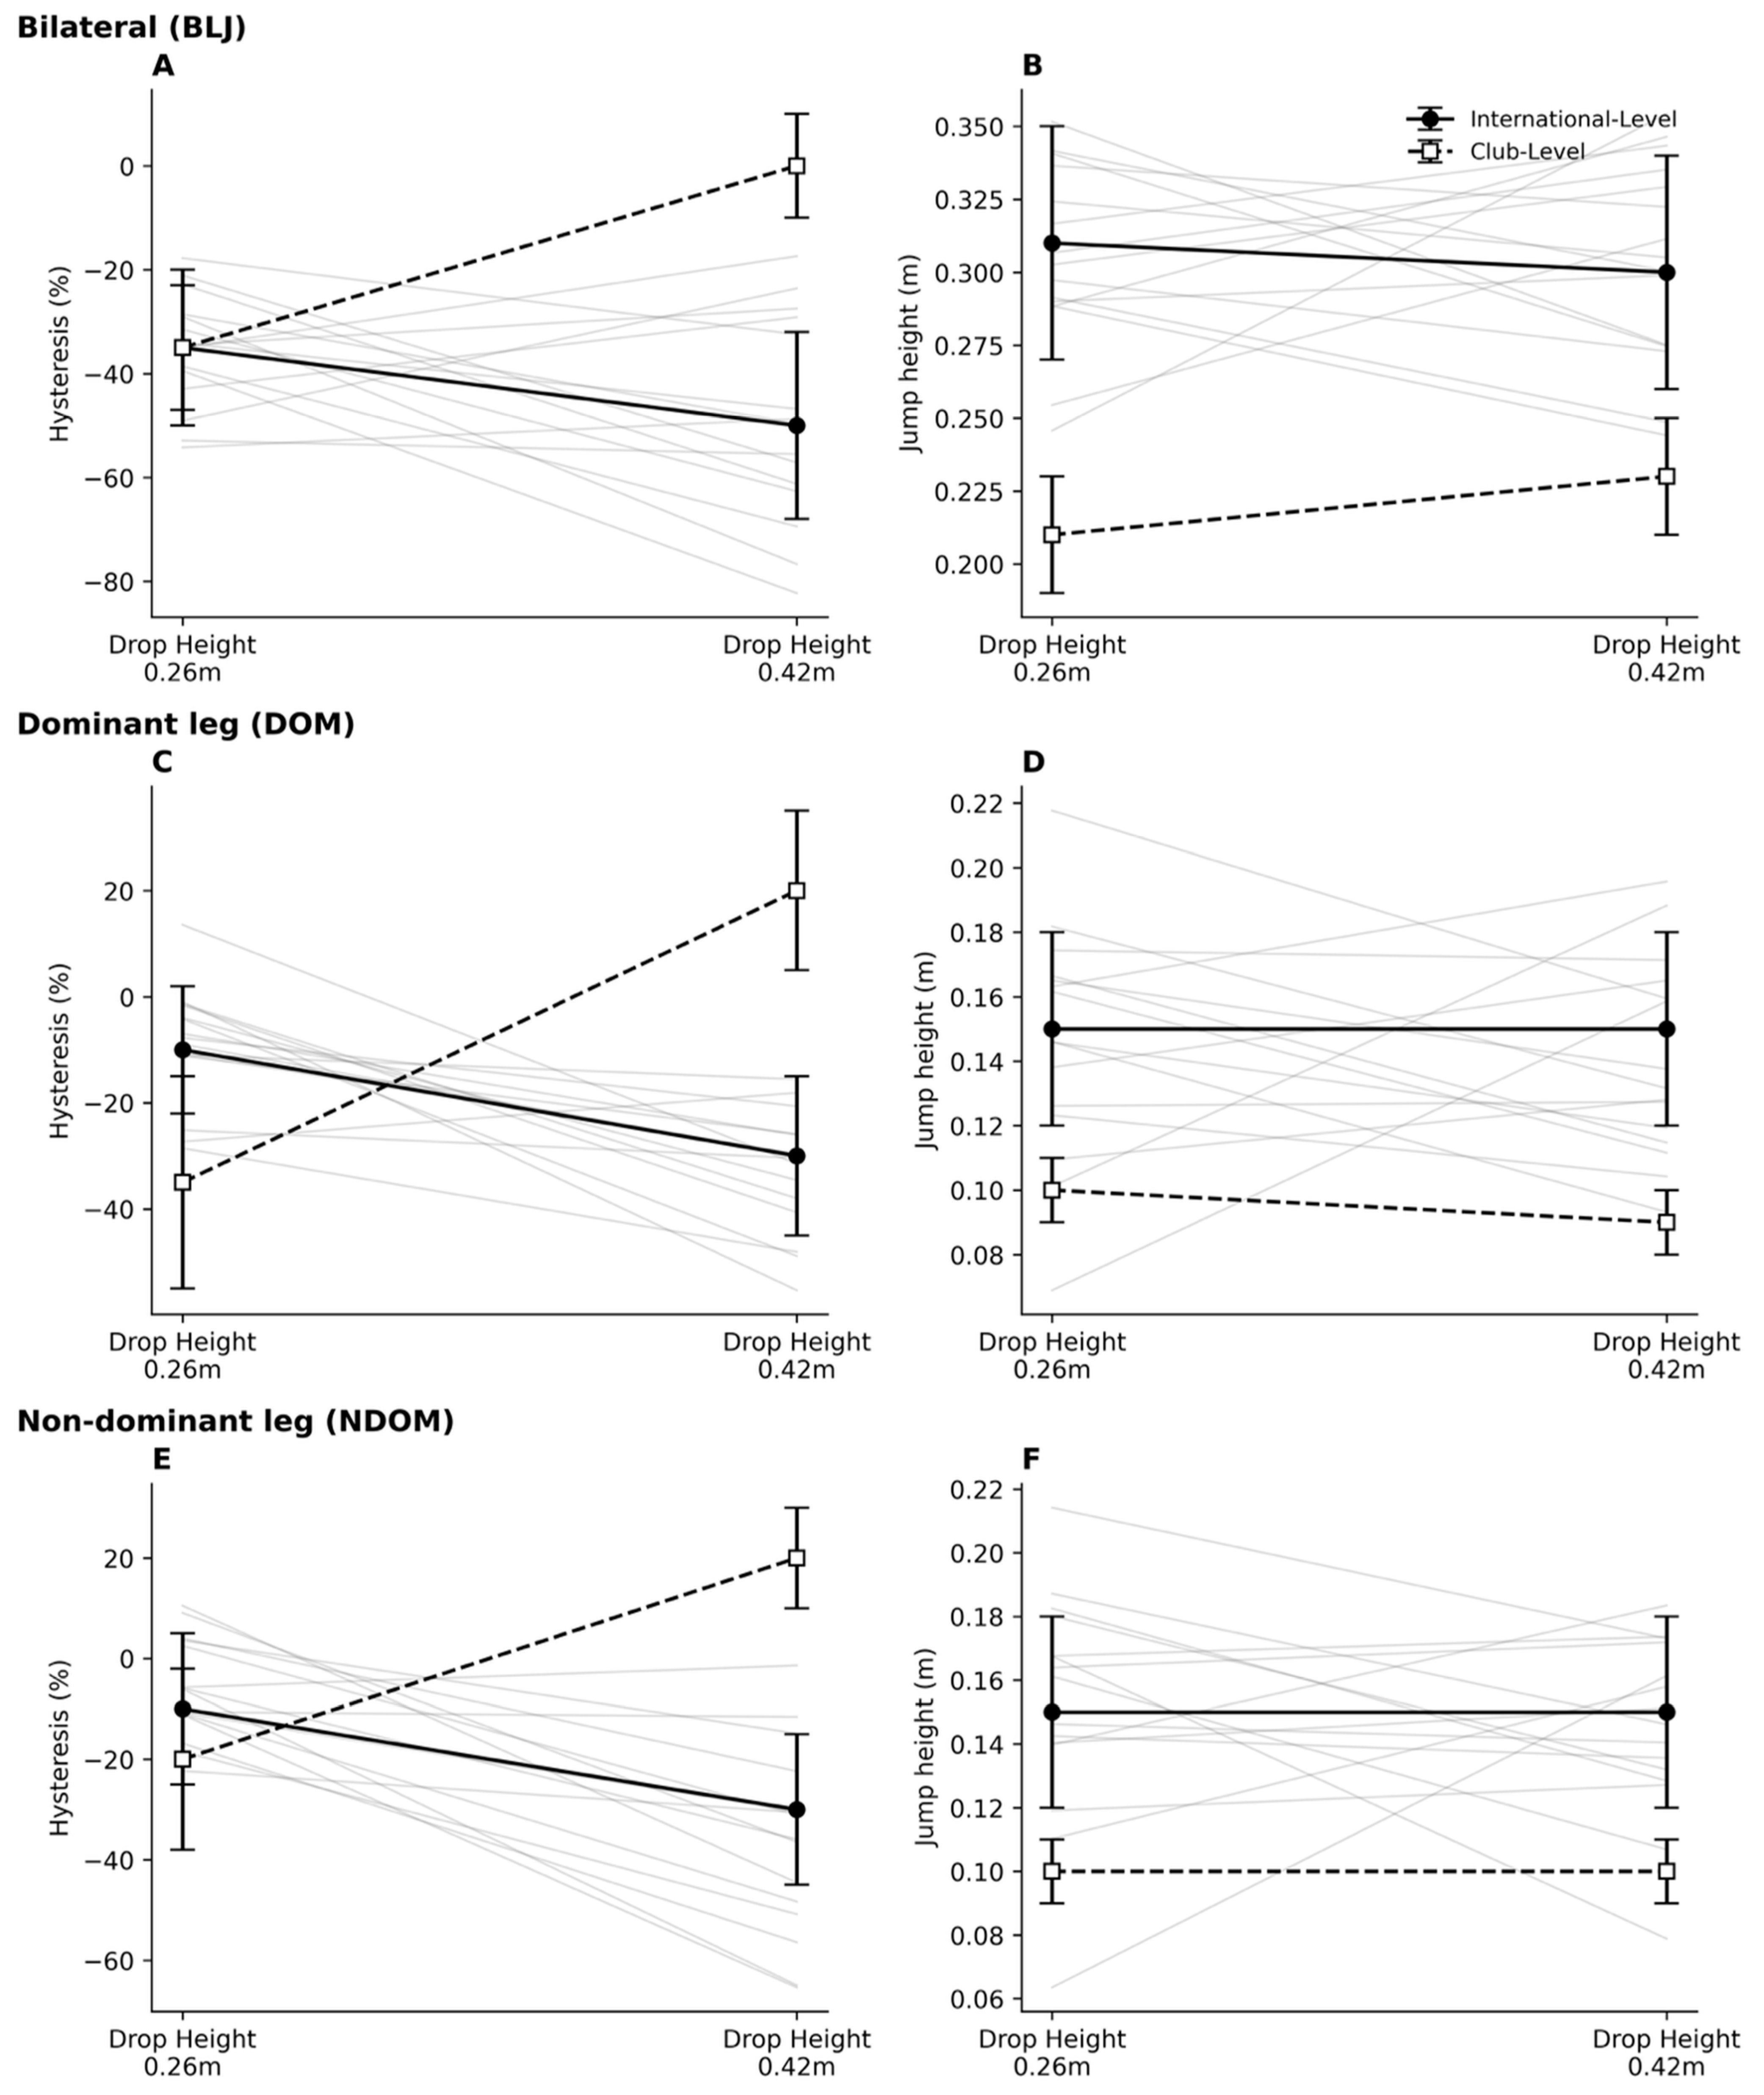
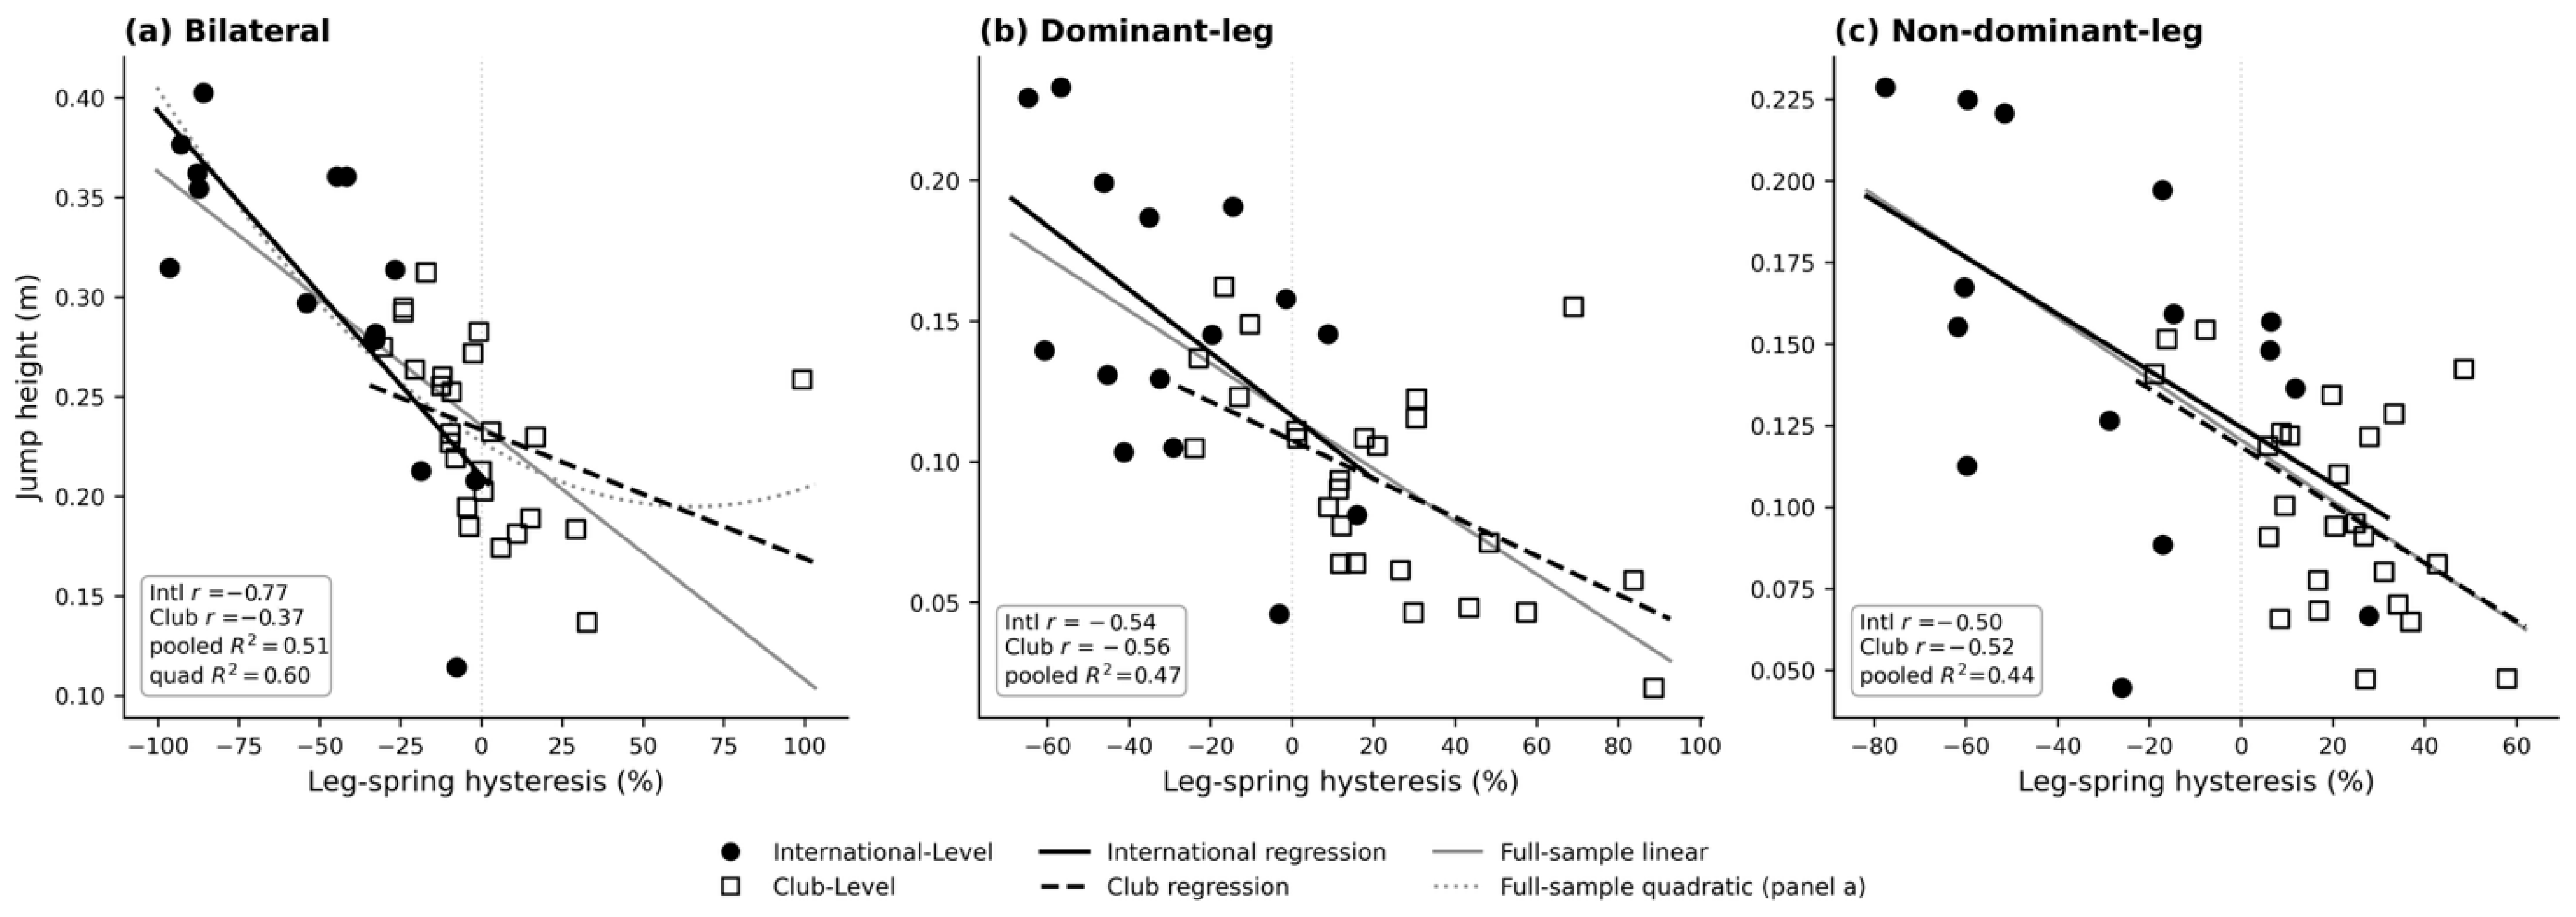

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.