


Simple Summary
Honey bees (Apis mellifera L.) play a vital role in the pollination of different crop plants but remain exposed to lethal and sub-lethal doses of pesticides which are used in different farming systems. This study investigated how the indirect individual dietary trophic exposure of two commonly used insecticides, bifenthrin and acetamiprid, belonging to two different groups (pyrethroid and neonicotinoid), affect bee colonies. Sunflower fields (Hysun-33) were subjected to different sub-lethal doses of these insecticides. After seven days of individual insecticidal treatments, twenty-seven bee colonies were introduced at nine different sites in these fields. The isolation distance between each site was not less than 3 km. The colonies introduced in the insecticide-free plots were considered as untreated control (T0). The results revealed that the bee colonies exposed to higher individual doses of insecticides exhibited less foraging activity, weaker social behaviors such as food sharing and communication, and shorter lifespans compared to the untreated control colonies. However, the growth durations of different immature stages of bees (egg, larva, and pupa) were not affected by the individual exposure of these insecticides. These findings suggest that even small amounts of pesticides taken through contaminated food can disturb the normal behavior and health of honey bee colonies. The results highlighted the need to use pesticides more precisely, especially by adjusting their timing and application methods, to protect pollinators that serve as an essential component of crop production and ecological sustainability.
Abstract
Apis mellifera L. is an important pollinator of both wild and domesticated crop plants, thus greatly contributing to plant biodiversity and commercial agriculture. However, in field conditions, honey bees remain exposed to different pesticides which ultimately affect colony health parameters and their associated ecological services. In the current study, the individual toxicities of sub-lethal doses of two distinct insecticides (bifenthrin and acetamiprid) belonging to different groups (pyrethroid and neonicotinoid) were assessed against the foraging activity, social interactions, and longevity of A. mellifera. The bees were exposed to individual doses of both insecticides via the dietary trophic route through contaminated pollen and nectar under natural field conditions. Sunflower crop (Hysun-33) was sown at nine different sites with an isolation distance of 3 km, and was treated with different doses (1/2, 1/4, 1/10, and 1/20 of the recommended field doses) of both insecticides. However, the untreated control crop plots were not subjected to any chemical treatments (bee colonies received no insecticide, and served as the baseline for making comparison). Twenty-seven bee colonies were introduced in these sites after seven days of treatment applications. Significant differences were observed in the foraging activity of A. mellifera (including bees going out from the hive, returning foragers, and those carrying pollens). The fecundity, adult longevity, and social behaviors like trophallaxis and antennation were significantly lower in bees exposed to higher individual insecticidal concentrations. However, the hatching duration, larval duration, and pupal duration were not affected by the tested insecticidal treatments. Overall, these findings demonstrate that the dietary trophic exposure of sub-lethal doses of insecticides compromised colony activities, which is indeed a matter of concern regarding the existing pesticide application methods in different agro-ecosystems. Such impacts may ultimately impair the survival of colonies, particularly when bees remain exposed to these chemicals over an extended period of time. Therefore, future studies must consider the pesticide application techniques and their application timing to mitigate the direct and indirect negative impacts of pesticides on pollinators.
1. Introduction
Apis mellifera L. contributes significantly in the pollination of over 70% of the crop species worldwide [1,2]. Their pollination services not only support plant biodiversity but also improve crop growth and yield. Bees are an important contributor of small- and large-scale commercial farming systems, adding billions of dollars annually to global agricultural economies [1,3]. The market value of a vast number of high-valued crops depends on their pollination services, which makes bees an essential component of different food production systems and rural livelihoods [4,5]. However, for the last few years, bees are experiencing severe population declines, which not only compromises their ecosystem services but also poses serious implications for food and nutritional security across the globe [6,7].
Apis mellifera is an important pollinator, which spends most of its time in vegetation to find different food resources for efficient brood development [8]. The health and development of a bee colony is maintained through trophallaxis, antennation, and division of labor, which not only regulate the flow of resources and information, but also make colonies more resilient against different environmental changes [9]. Different biotic and abiotic stressors such as habitat destruction, pathogen invasion, and pesticidal exposure pose a serious threat for bee colonies and their associated pollination services [10,11]. Although the causes of honey bee decline may be complex and interrelated, the widespread use of different pesticides in agro-ecosystems has been considered a potential contributing factor [12,13].
Insecticides, fungicides, and herbicides are mostly used as pesticides to safeguard crops from different biotic stressors. However, their widespread use has also contaminated the agricultural landscapes, which poses serious threats for pollinators and other non-target organisms [14,15]. Synthetic insecticides such as bifenthrin, belonging to the group of pyrethroids, are preferred in different agro-ecosystems due to their quick mode of action against different insect pests [16]. Similarly, acetamiprid, a neonicotinoid, binds with nicotinic acetylcholine receptors of the insect nervous system, leads to overstimulation of the nervous system, and compromises insect vital body functions, leading to the death of the organism [17,18]. However, despite being regarded as less toxic in comparison to other neonicotinoids, sub-lethal exposure of acetamiprid is also capable of disrupting learning, olfactory memory, and social recognition in honey bees [19]. It has been reported that the systemic properties of most of the modern-day insecticides facilitate their translocation to nectar and pollen, which might later contaminate honey bees, mainly through feeding [20].
Honey bees, mainly foragers, are more prone to infield pesticidal exposure, due to their foraging flights, compared to in-hive nurse bees [21]. The bees endure pesticides in various ways, mainly through contaminated nectar, pollen, water, and other hive material [22]. Moreover, trophic transfer via diet occurs when the accumulated pesticide residues in food sources impact the entire colony [23]. Pesticide residues passed through trophallaxis and jelly induce sub-lethal effects on the health and reproduction of bees [24,25]. The exposure to sub-lethal doses of pesticides usually does not lead to immediate death, but affects certain physiological and behavioral aspects of bees, which results in decreased foraging efficiency, navigation, social homeostasis, and immune competence, thus weakening the survivability of a colony [26,27]. Moreover, low or sub-lethal concentrations of bifenthrin and other insecticides interfere with learning, memory, and social behaviors like trophallaxis and grooming of honey bees. These disruptions influence the foraging patterns and intra-colony communication that are vital for the homeostasis of the colony [28,29]. Antennal contact, trophallaxis, and grooming all play important roles in communication and exchange of information, food and pheromones. These behaviors guarantee integration in the colony and adaptive responses against stressors [30]. Sub-lethal exposure to pesticides also impairs queen physiology, decreases its fecundity, and changes pheromone synthesis, which has an adverse impact on the reproduction of the colony and behavior of the worker bees [31,32,33].
Pesticidal exposure also reduces brood viability by compromising the quality of the brood feed, which results in production of a smaller and less viable worker population [24,34]. Decreased fecundity and brood survival of queens not only reduce the growth of colonies, the size of workforce, and the output of honey, but also endangers the sustainability of colonies and pollination services [35,36,37]. Reduced reproduction and colony strength limits pollination services, underscoring the need to assess the sub-lethal effects of pesticides on honey bees [11]. Field-based experiments that incorporate environmental factors and realistic exposure pathways provide more precise estimates of how pesticides influence colony performance and social behavior of honey bees [38].
Most of the previous literature largely remained focused on exploring the impacts of direct contact or acute toxicity of pesticides on honey bees. However, the trophic exposure route of pesticides (via contaminated nectar or pollen, or through their food) remains largely underexplored, particularly concerning its effects on foraging activity, social behavior, and bee longevity [24]. This study introduces a novel perspective in honey bee toxicology by examining the sub-lethal trophic (dietary) pathway of insecticide exposure instead of conventional toxicity routes (direct or surface residual). It investigated the trophic effects of sub-lethal concentrations of two popular insecticides, i.e., bifenthrin (a pyrethroid) and acetamiprid (a neonicotinoid) on A. mellifera in field-relevant conditions. The work is distinguished from its counterparts by its field-scale experimental design, integration of multiple behavioral and social endpoints (foraging activity, trophallaxis, antennation, and longevity), and the comparative assessment of two insecticide classes. These findings enhance knowledge of how long-term, low-level dietary exposure of insecticides can influence colony dynamics, individual bee behavior, and ultimately pollination performance and colony sustainability.
2. Materials and Methods
2.1. Experimental Design and Colony Setup
The current experiment required meticulous observations and therefore involved an independent designated field area which can be controlled over certain variables as per study requirements. The selected fields fulfilling the above requirements belong to the Apiculture Research Field, Department of Entomology, The Islamia University of Bahawalpur (Punjab, Pakistan). The study also involved twenty-seven homogenized, healthy, proportionately similar, and disease- and pest-free bee colonies (A. mellifera ligustica) with fertile queen bees. The bee colonies were kept in hives and equally aligned regarding adult bee population, colony strength, and brood area. All the queens, obtained from a single source colony, were fertile and of similar age. This standardization minimized the chances of variability among colonies and ensured that the observed effects were primarily related to insecticide exposure rather than initial colony differences [39]. Initially, the bee colonies were maintained at the Apiculture Research Area, The Islamia University of Bahawalpur. During this colony maintenance period, the foraging sources within a 3 km vicinity of the Apiculture Research Area were not subjected to any chemical treatments. The hive chambers were checked regularly to ensure that bees were performing in the best possible way as a healthy colony.
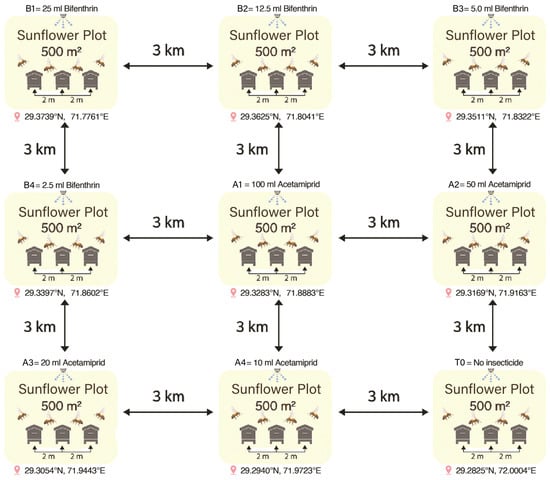
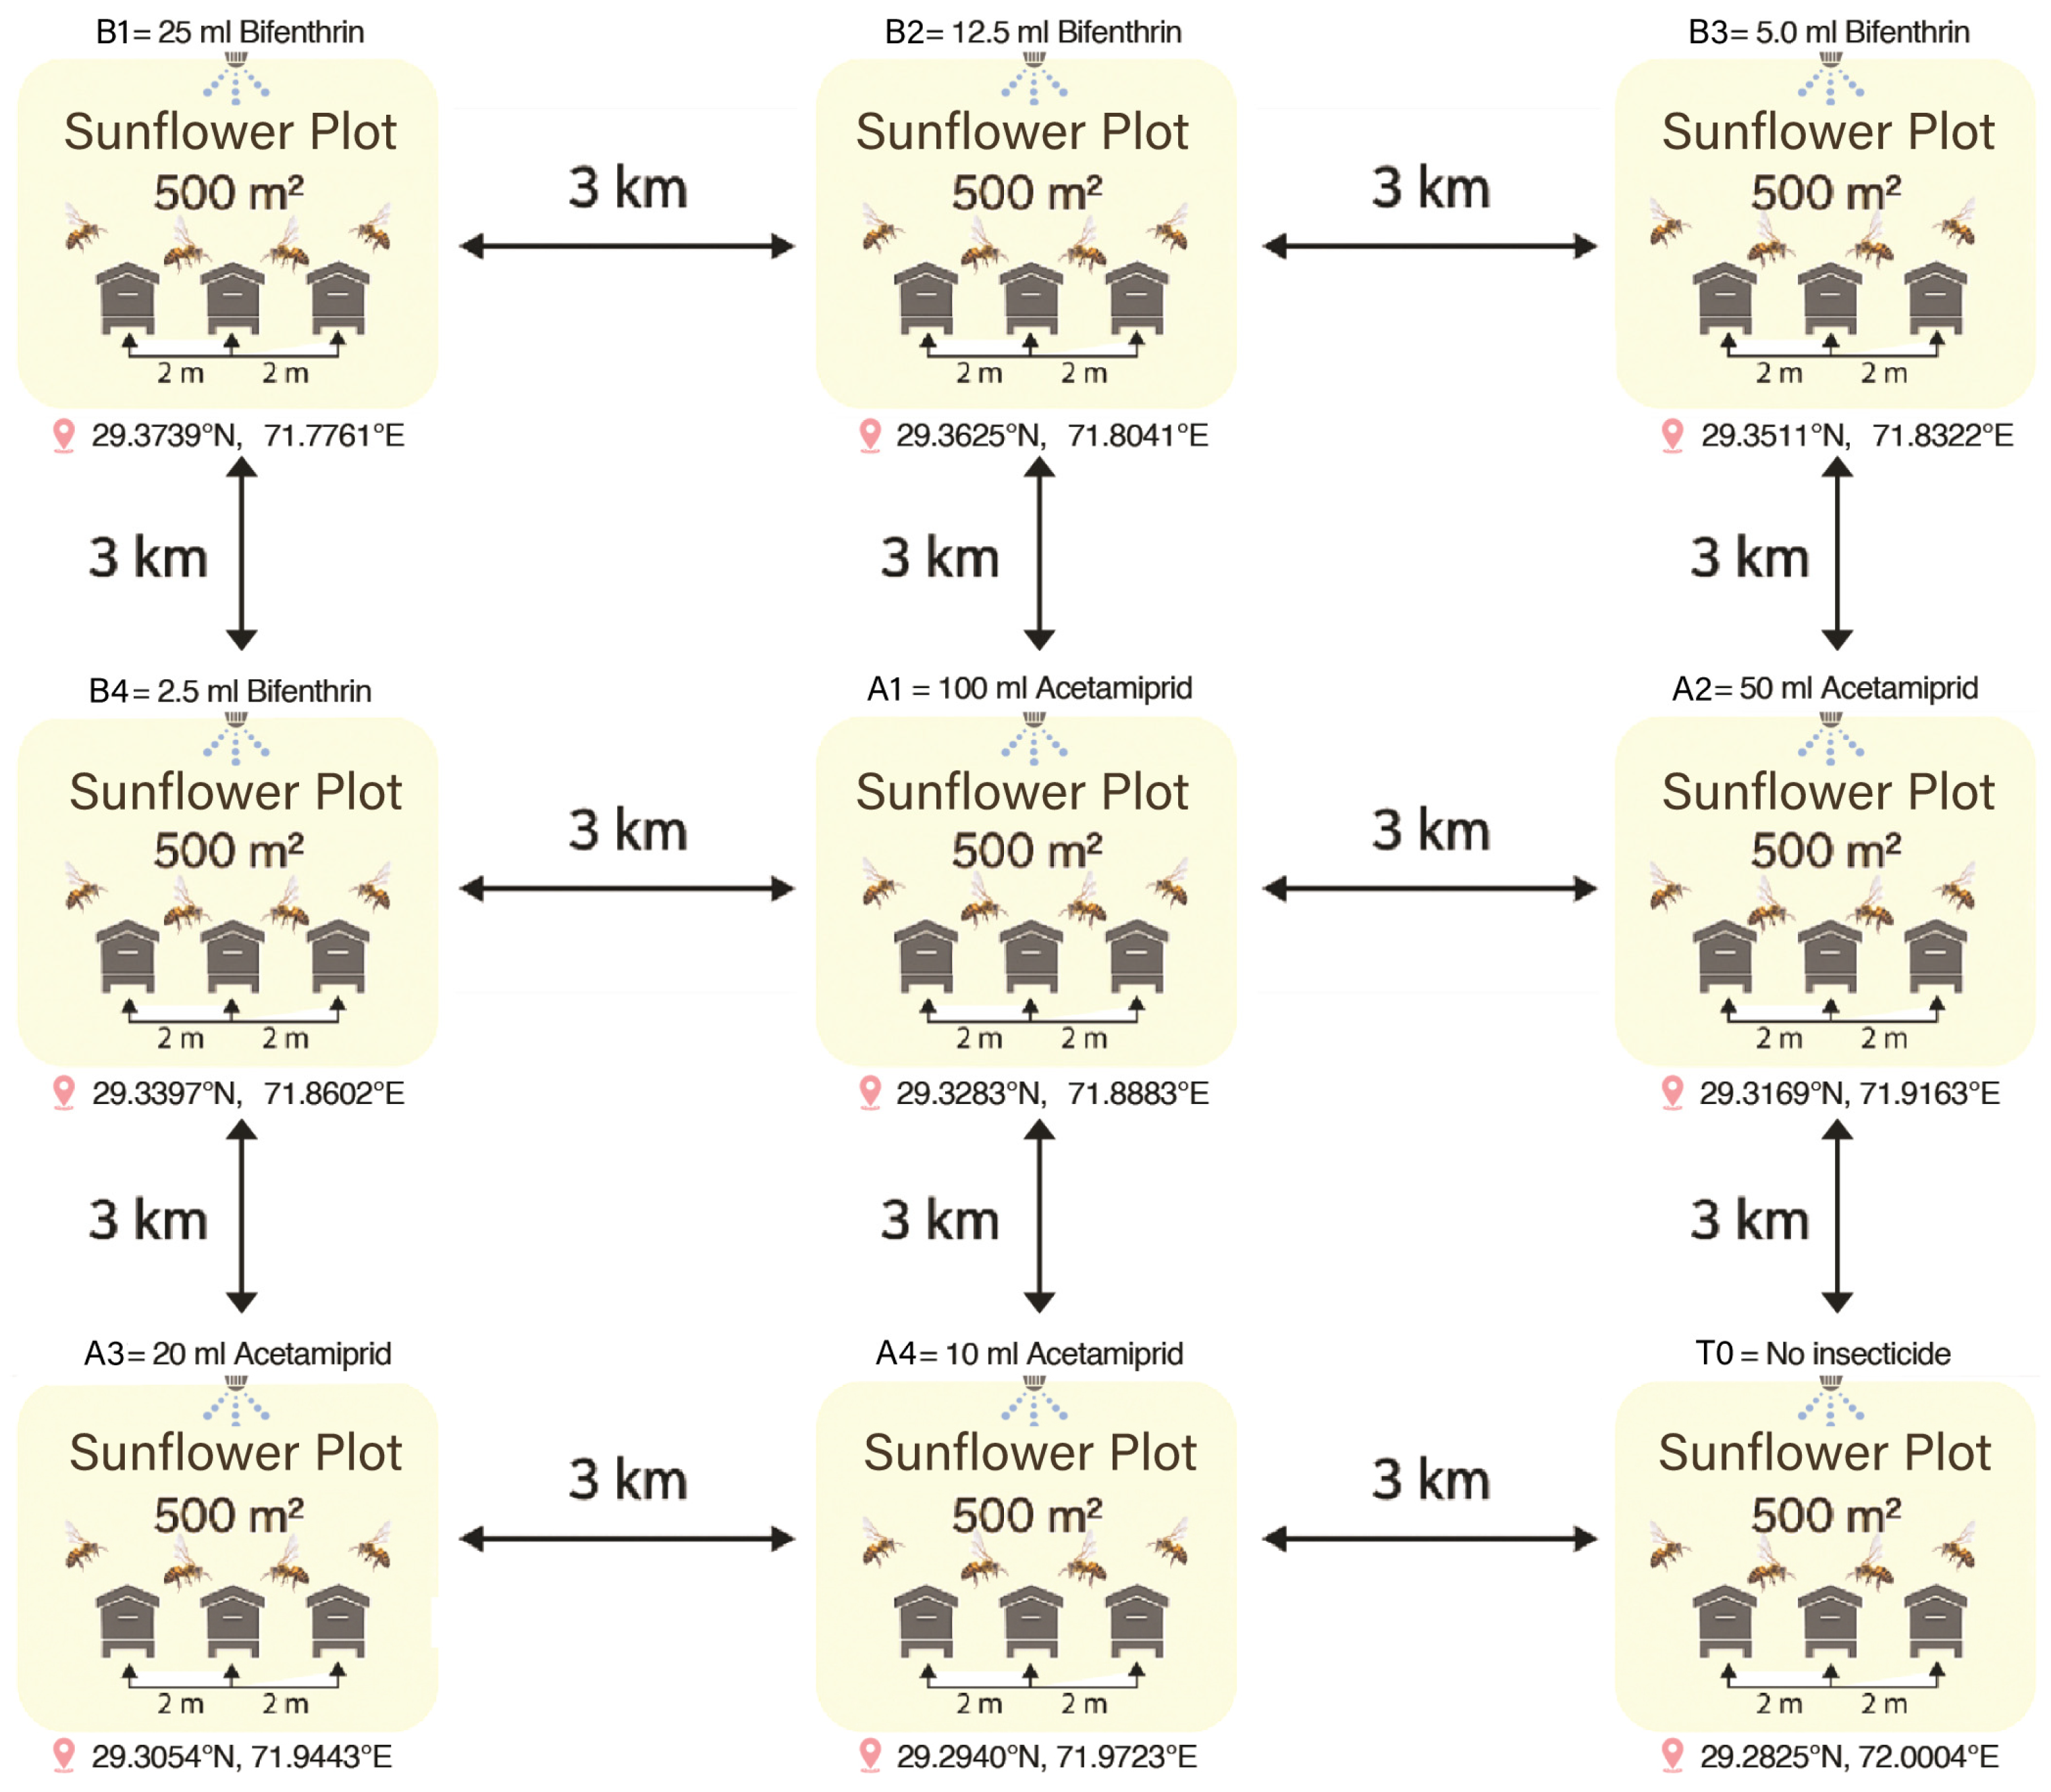
Sunflower (Hysun-33) was planted in the last week of January 2023 at nine different locations (plots) (29.3739° N, 71.7761° E; 29.3625° N, 71.8041° E; 29.3511° N, 71.8322° E; 29.3397° N, 71.8602° E; 29.3283° N, 71.8883° E; 29.3169° N, 71.9163° E; 29.3054° N, 71.9443° E; 29.2940° N, 71.9723° E; 29.2825° N, 72.0004° E) of the Apiculture Research Field, each with an area of 500 m2. The crop was subjected to all required agronomic practices to maintain a healthy stand. The area (500 m2) was deemed enough to rear three honey bee colonies [40]. The foraging range of honey bees is reported to be 1.5–2 km [41,42]; therefore, each crop plot was kept 3 km apart to prevent foraging overlap among bee colonies (Figure 1). Sunflower flowering commenced in the second week of March 2023, marking the initiation of the experimental phase. The average temperature of the experimental site ranged between 28 and 34 °C, with relative humidity around 45–55%. No significant rainfall was recorded during the experimental period, providing favorable conditions for foraging activity. Moreover, before the execution of the experiment, meetings were organized with farmers to ensure that no insecticides were applied on plots near the experimental vicinity. Spraying of both insecticides was conducted according to a pre-planned schedule on the 3rd, 4th, and 5th of April 2023, with three plots treated each day. The data from each plot was collected after similar time intervals of insecticidal applications to avoid any experimental error.
Figure 1.
Systematic diagram showing the placement of 27 bee colonies and sunflower crop fields. Each plot (500 m2) was separated from the others by a minimum distance of 3 km, while three bee colonies were placed within each sunflower field at 2 m spacing from each other.
2.2. Preparation of Sub-Lethal Doses of Tested Insecticides
The commercial formulations of Bifenthrin 10 EC (Talstar® 10 EC, FMC Corporation, Philadelphia, PA, USA) and Acetamiprid 20 SP (Acelan® 20 SP, FMC Corporation, Philadelphia, PA, USA) were obtained from a local pesticide market. To simulate oral trophic exposure via contaminated nectar and pollen, bee colonies were introduced in the insecticide-treated sunflower plots after one week of spraying to avoid any direct contact with insecticide treated plant surfaces. In this case, bees could only be exposed to insecticidal treatments via contaminated pollen or nectar through the dietary pathway [43,44]. The insecticides were applied on the sunflower crop at the flowering stage using a knapsack sprayer, following standard field application protocols [45]. Sub-lethal doses of insecticides were prepared by diluting the recommended field rates of Bifenthrin (50 mL/500 m2) and Acetamiprid (200 mL/500 m2) in water. Four treatments for each insecticide were prepared: one-half (B1 and A1), one-quarter (B2 and A2), one-tenth (B3 and A3), and one-twentieth (B4 and A4) of the recommended doses. A control treatment (T0) with no insecticide was also included. The specific amounts of insecticides applied per 500 m2 plot are provided in Table 1.
Table 1.
Description of treatments, dose preparations, and insecticide amounts (mL) applied per 500 m2 area for trophic toxicity assessment of Bifenthrin 10 EC and Acetamiprid 20 SP against A. mellifera (n = 3 colonies per treatment).
2.3. Foraging Activity
The foraging activity of the bees was determined by visual observation, i.e., by counting the bees present in the hive following the method adopted by Islam et al. [39]. The numbers of bees going out of the hive for foraging [46], returning back to their hives [47], and those carrying pollen on their legs, were recorded for 5 min [48] between 8:00 to 10:00 a.m. The mentioned time period corresponds to peak foraging activity of A. mellifera, as documented in previous studies [49,50].
2.4. Social Interaction
In the social behavior experiments, two forms of bee behaviors, i.e., antennation and trophallaxis, were assessed. The hives were regularly monitored with high-pixel cameras, Go-Pro Hero (CHDRB-101-CN), GoPro, Inc., San Mateo, CA, USA. The cameras were installed at a fixed and identical position facing the central brood frame of all colonies, where social interactions are most frequent. The camera setup was standardized across all beehives and remained unchanged throughout the observation period to ensure minimal disturbance among colonies. A non-intrusive low-intensity light was used to light up the hive so that the camera could get high-quality footage without disturbing the bees. The source of light was also placed strategically to avoid any direct contact with the bees and so as to reduce any kind of stress or behavioral alterations [51]. Videos were recorded for a total of 30 min, divided into three 10 min sessions. Antennation and trophallaxis are rapid and frequent behaviors, and therefore can be reliably quantified within such short observation windows [39,52,53,54]. The recorded footage was subsequently analyzed for obtaining precise results.
2.5. Longevity
To measure dietary trophic effects in all the experimental colonies, empty frames containing wax only were placed in the center of the hive, in which the number of eggs laid by the queen bee were counted [55]. The data regarding egg counts was taken for 5 days. After that, the counted number of eggs was labeled to observe their successful transformation into the pupae and locate broods in the hives. The eggs laid by the queen were tagged and observed for egg hatching period, larval period, and pupal period. Once the adult workers emerged, they were marked using POSCA color marker (non-toxic marker) (POSCA PC-5M, Mitsubishi Pencil Co., Ltd., Boulogne-Billancourt Cedex, Boulogne-Billancourt, France) on their thorax [49,56], and monitored daily in the morning at 10 am, until they died or were found missing. The identified bees were counted and the adult longevity data for all tested treatments were recorded [57].
2.6. Statistical Analysis
Statistical analyses were performed using R software (version 4.3.0). The data regarding experimental parameters, such as foraging activity (bees left, returning bees, pollen collection), and longevity indicators (fecundity, hatching period, larval period, pupal period, and adult lifespan were analyzed under Randomized Complete Block Design (RCBD), while one-way analysis of variance (ANOVA) under Complete Randomized Design (CRD) was applied for data regarding social interactions (trophallaxis frequency and antennation frequency). The significance of differences between treatment means was established through the Least Significant Difference (LSD) test at 5% significance level. Data was pre-tested to ensure that the data were normally distributed (Shapiro–Wilk test) and had equal variances (Levene’s test). There was no need for data transformation, as the assumptions were met. Pearson correlation analysis between trophallaxis and antennation frequencies was performed in R to assess the strength and direction of their linear relationship. To visualize and compare the treatment effects, all graphs were generated using the ggplot2 package (version 3.5.1) and dplyr package (version 1.1.4), while for correlation analysis, the corrplot package (version 0.95) was used in the same software.
3. Results
3.1. Foraging Activities
3.1.1. Bees Leaving Hive
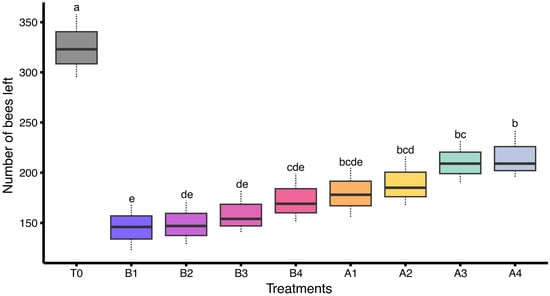
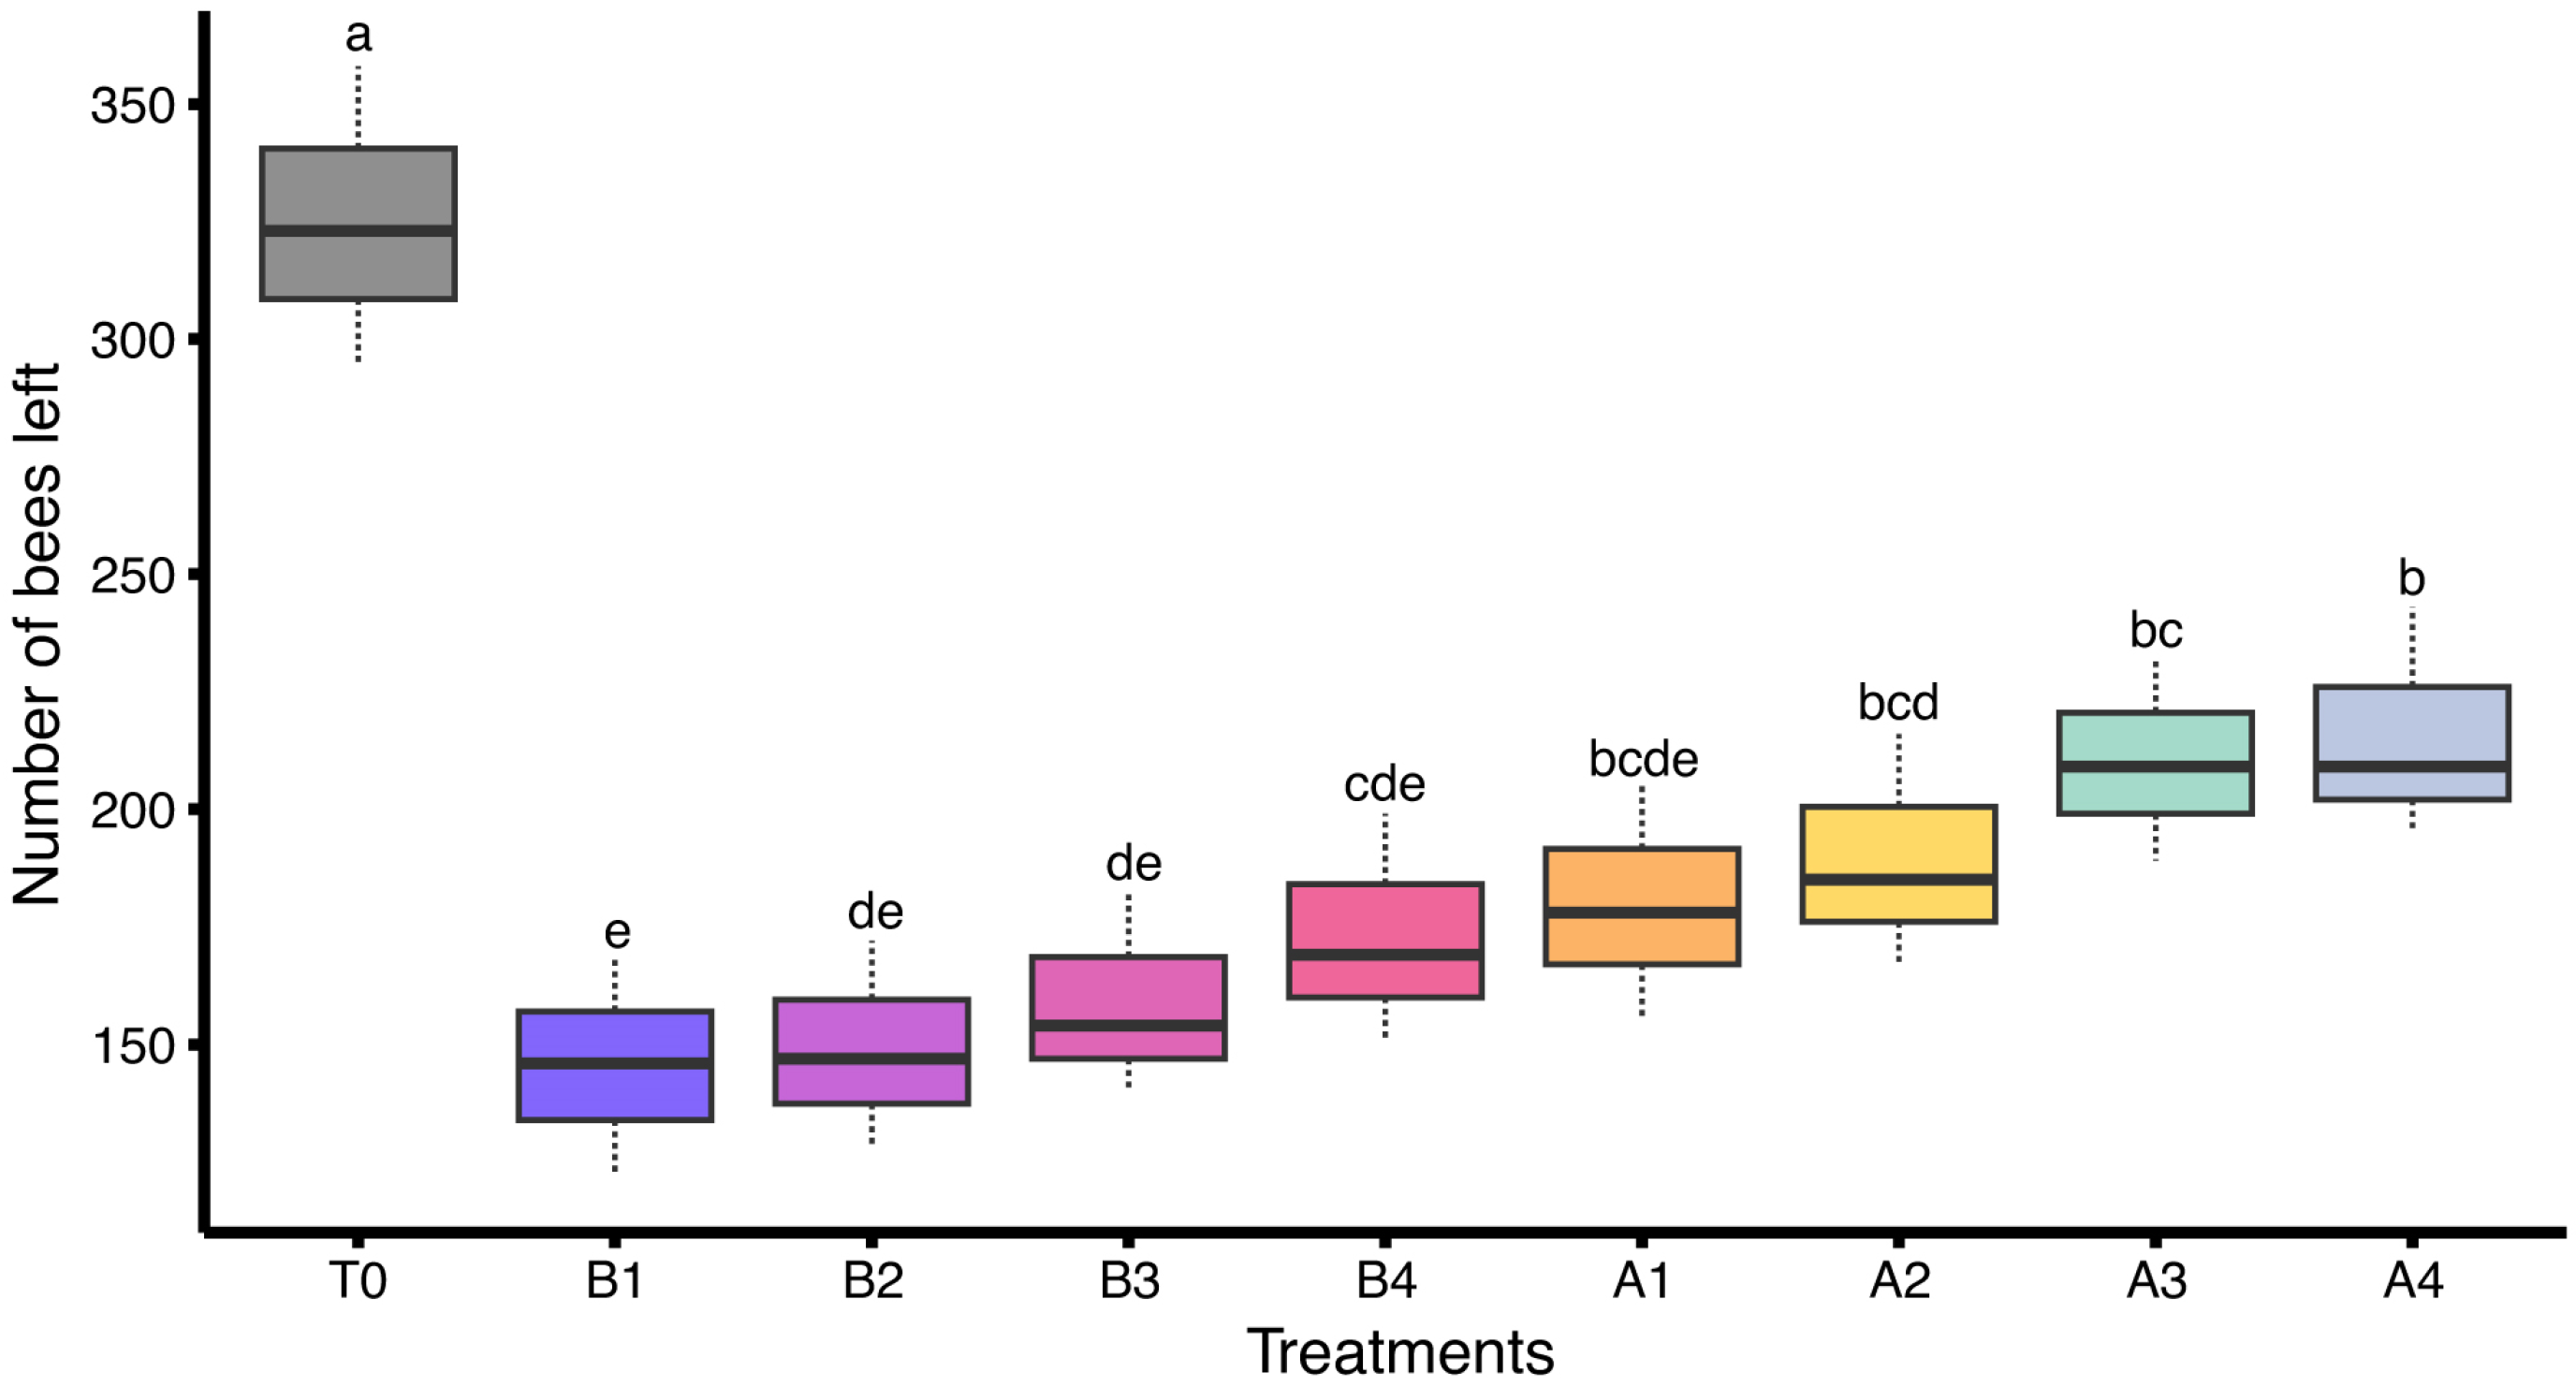
A statistically significant difference was observed in the number of bees leaving the hive among colonies exposed to different insecticide treatments under field conditions (F(8,18) = 15.1, p < 0.05). The highest bee population leaving the hive was recorded in the control group (T0: 325.00 ± 18.50 bees). Colonies treated with A4 (215.67 ± 14.25 bees) and A3 (210.00 ± 12.42 bees) showed moderate numbers of bees leaving the hive, whereas lower populations were observed in A2 (189.33 ± 14.31 bees), A1 (179.67 ± 14.17 bees), and B4 (173.00 ± 14.00 bees). The lowest bee populations leaving the hive were recorded in colonies subjected to B3 (159.00 ± 12.66 bees), B2 (149.00 ± 12.74 bees), and B1 (145.33 ± 13.28 bees). These results indicate a clear dose-dependent reduction in foraging activity with increasing insecticide exposure (Figure 2).
Figure 2.
Number of bees leaving the hive in colonies subjected to different insecticides under field conditions (n = 3 colonies per treatment). Different letters indicate statistically significant differences among treatments based on LSD test at α = 0.05. The dashed lines (whiskers) above and below of each box represent data variability.
3.1.2. Bees Returning to the Hive
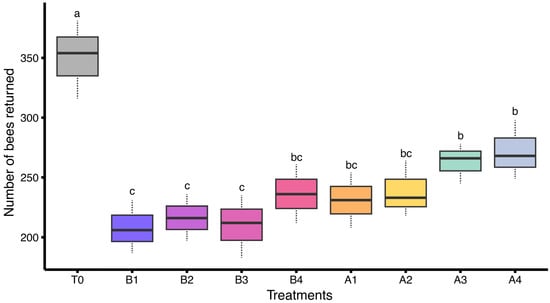
A statistically significant difference was observed in the number of bees returning to the hive among colonies exposed to different insecticide treatments under field conditions (F(8,18) = 10.3, p < 0.05). The highest number of returning bees was recorded in the control group (T0), with a mean of 350.33 ± 18.85 bees, reflecting the absence of chemical stress. Colonies treated with A4 (271.67 ± 14.26) and A3 (263.00 ± 9.64) showed moderate return numbers, while slightly lower numbers were observed in A2 (238.33 ± 13.54), B4 (236.33 ± 14.15), and A1 (231.00 ± 13.28). The lowest returning bee populations were recorded in colonies exposed to B2 (216.33 ± 11.26 bees), B3 (210.00 ± 15.04 bees), and B1 (208.00 ± 12.74 bees). This trend reflects reduced foraging efficiency and potential navigational impairment caused by insecticidal stress (Figure 3).
Figure 3.
Number of bees returning to the hive in colonies treated with various insecticides under field conditions (n = 3 colonies per treatment). Different letters indicate statistically significant differences among treatments based on LSD test at α = 0.05. The dashed lines (whiskers) above and below of each box represent data variability.
3.1.3. Bees Containing Pollens
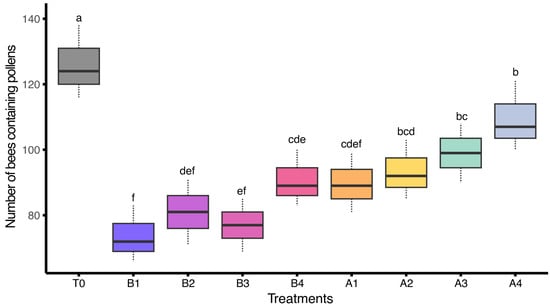
Similarly, the number of bees exposed to different insecticidal treatments under field conditions showed significant differences regarding bees that carried pollens in their legs (F(8,18) = 9.25, p < 0.05). The highest number of bees carrying pollens was recorded in the control group (T0) with a mean of 126.00 ± 6.43, indicating optimal foraging performance in the absence of chemical exposure. Colonies treated with A4 (109.33 ± 6.17) and A3 (99.00 ± 5.20) showed moderate pollen collection, while slightly lower values were recorded in A2 (93.33 ± 5.24), B4 (90.67 ± 4.98), and A1 (89.67 ± 5.21). The lowest number of bees carrying pollens was recorded in B2 (81.00 ± 5.77), B3 (77.00 ± 4.62), and B1 (73.67 ± 4.98). This pattern suggests that sub-lethal insecticide exposure negatively affects resource collection and foraging motivation (Figure 4).
Figure 4.
Number of bees carrying pollens, treated with various insecticides under field conditions (n = 3 colonies per treatment). Different letters indicate statistically significant differences among treatments based on LSD test at α = 0.05. The dashed lines (whiskers) above and below of each box represent data variability.
3.2. Social Interactions
3.2.1. Trophallaxis
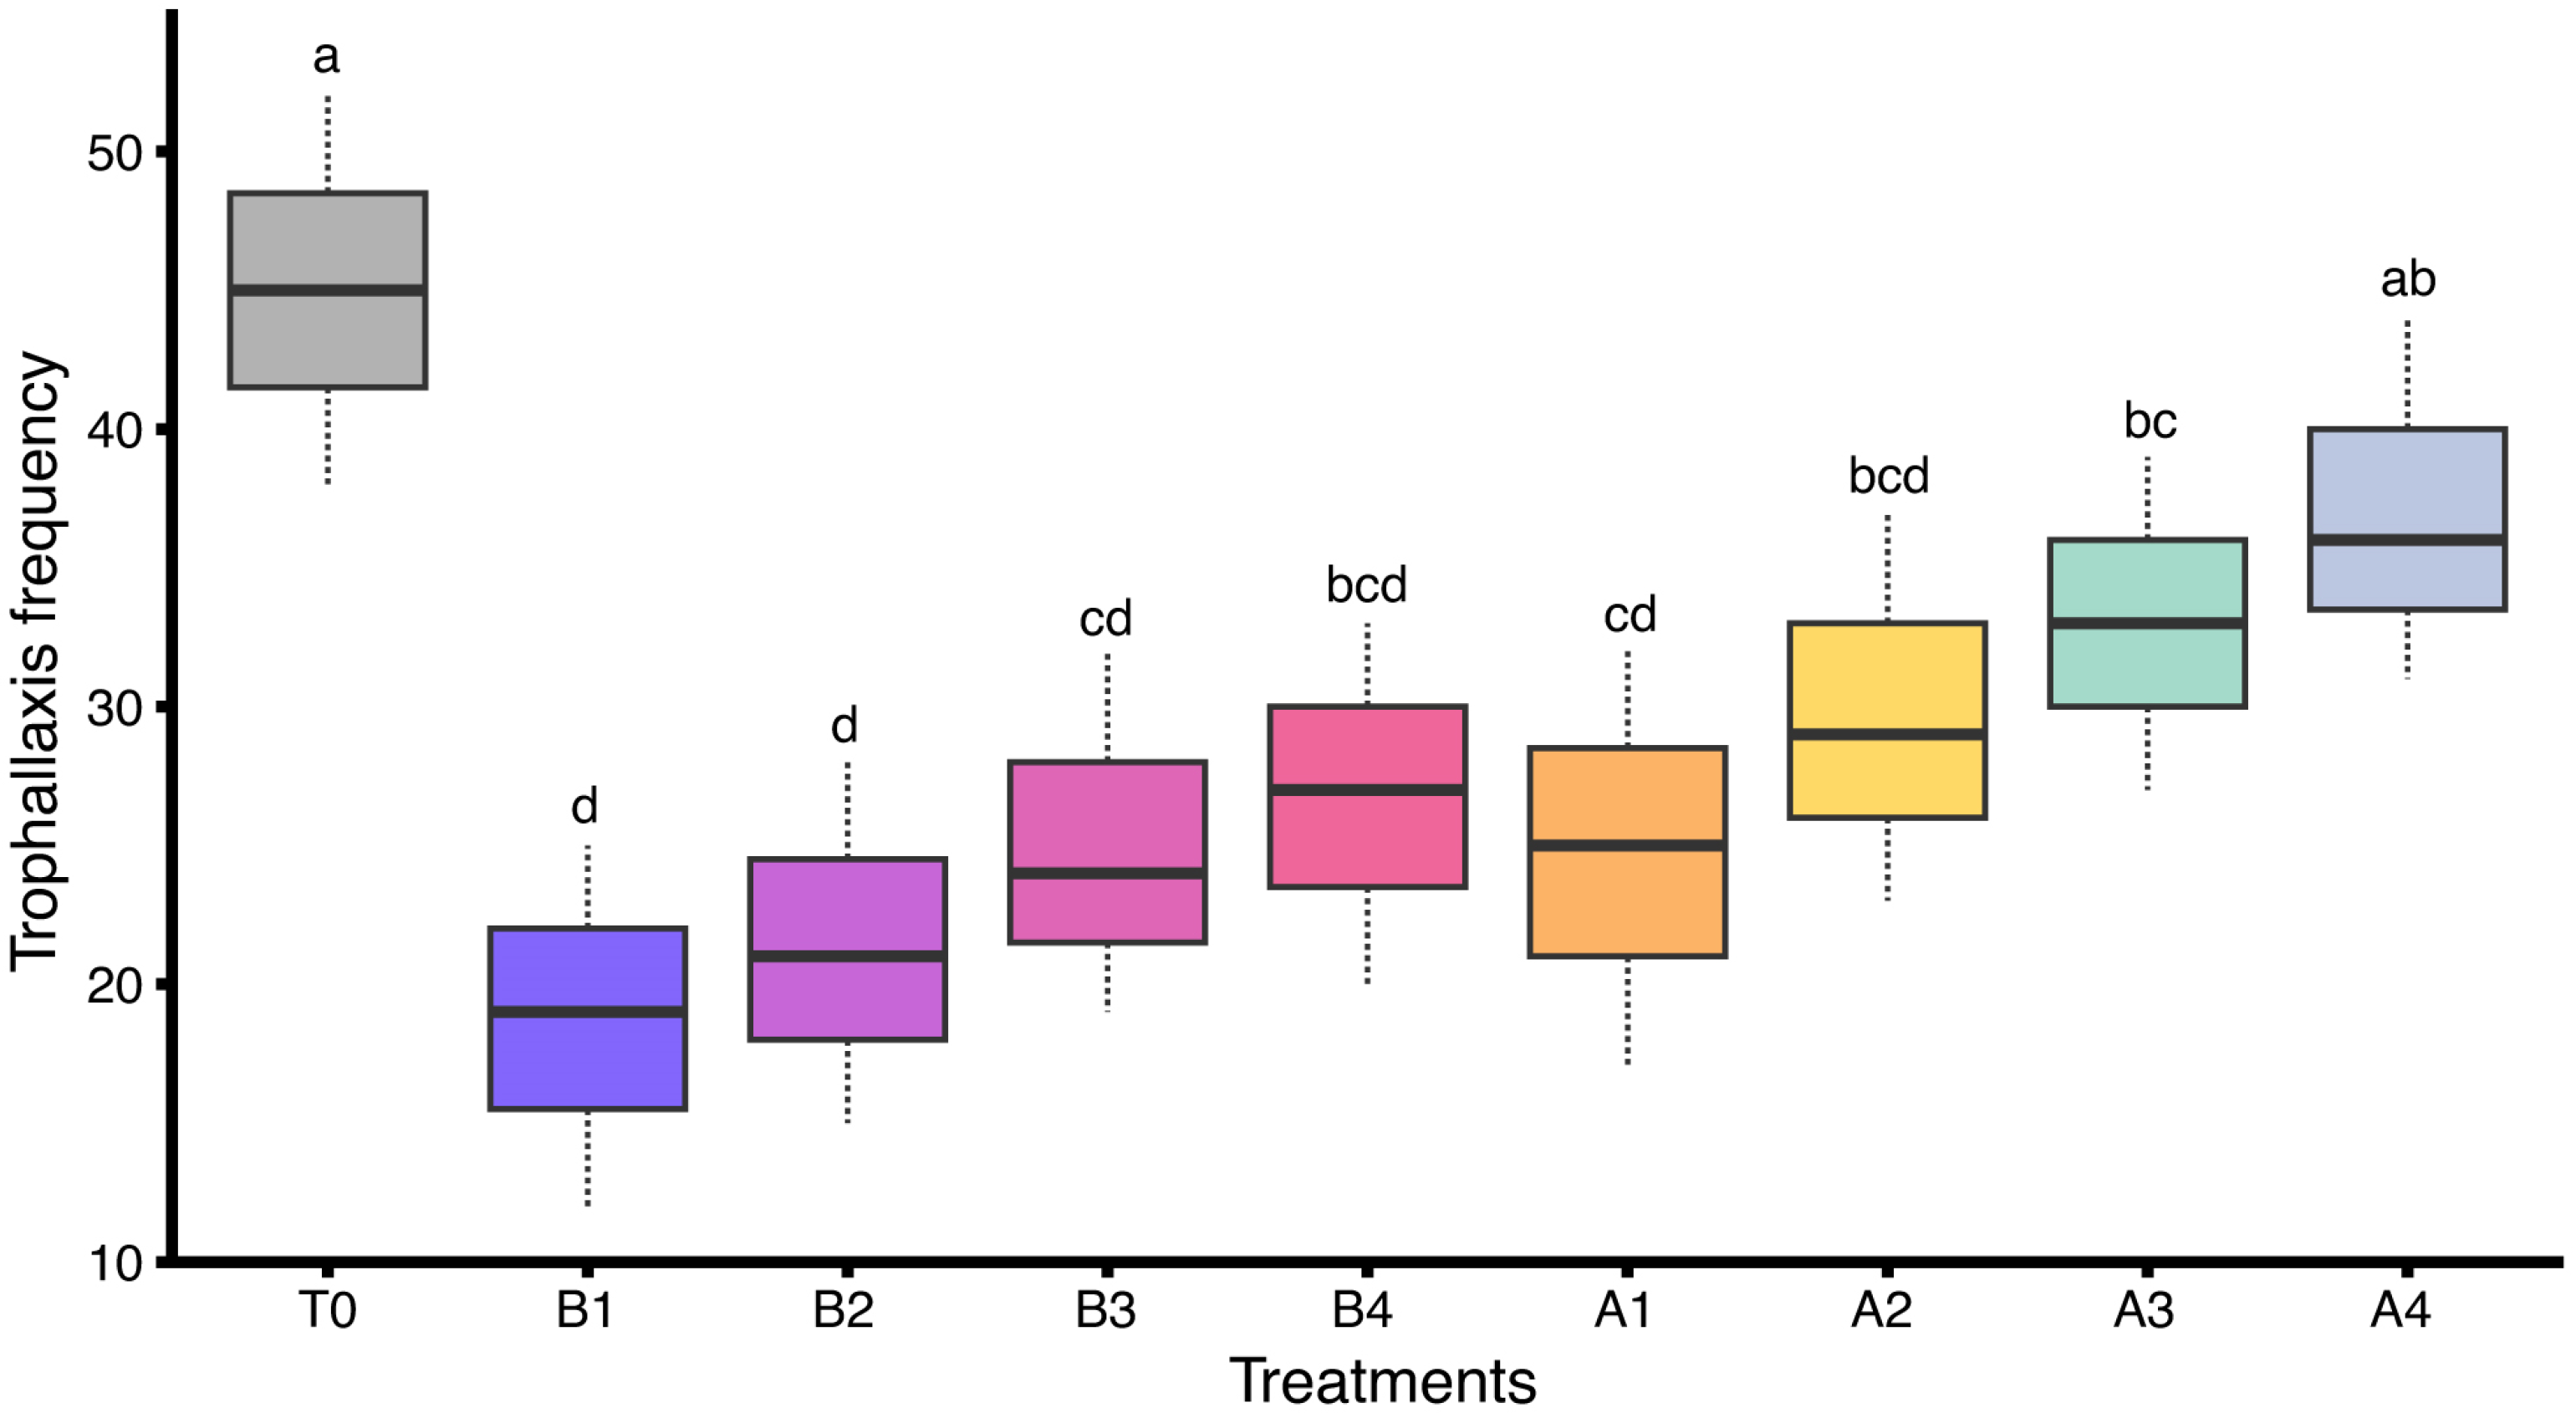
A statistically significant difference was observed in trophallaxis behavior of honey bee colonies subjected to different insecticide treatments under field conditions (F(8,18) = 4.53, p < 0.05). The control group (T0) had the highest mean frequency (45.00 ± 4.04), indicating active social food-sharing in the absence of chemical exposure. Moderate activity was observed in A4 (37.00 ± 3.79) and A3 (33.00 ± 3.46), while lower values were recorded in A2 (29.67 ± 4.06), B4 (26.67 ± 3.76), B3 (25.00 ± 3.79), and A1 (24.67 ± 4.33). The lowest trophallaxis frequencies were found in B2 (21.33 ± 3.76) and B1 (18.67 ± 3.76). This indicates that insecticide stress may impair trophallaxis behavior and intra-colony communication (Figure 5).
Figure 5.
Trophallaxis frequency in honey bee colonies treated with various insecticides under field conditions (n = 3 colonies per treatment). Different letters indicate statistically significant differences among treatments based on LSD test at α = 0.05. The dashed lines (whiskers) above and below of each box represent data variability.
3.2.2. Antennation
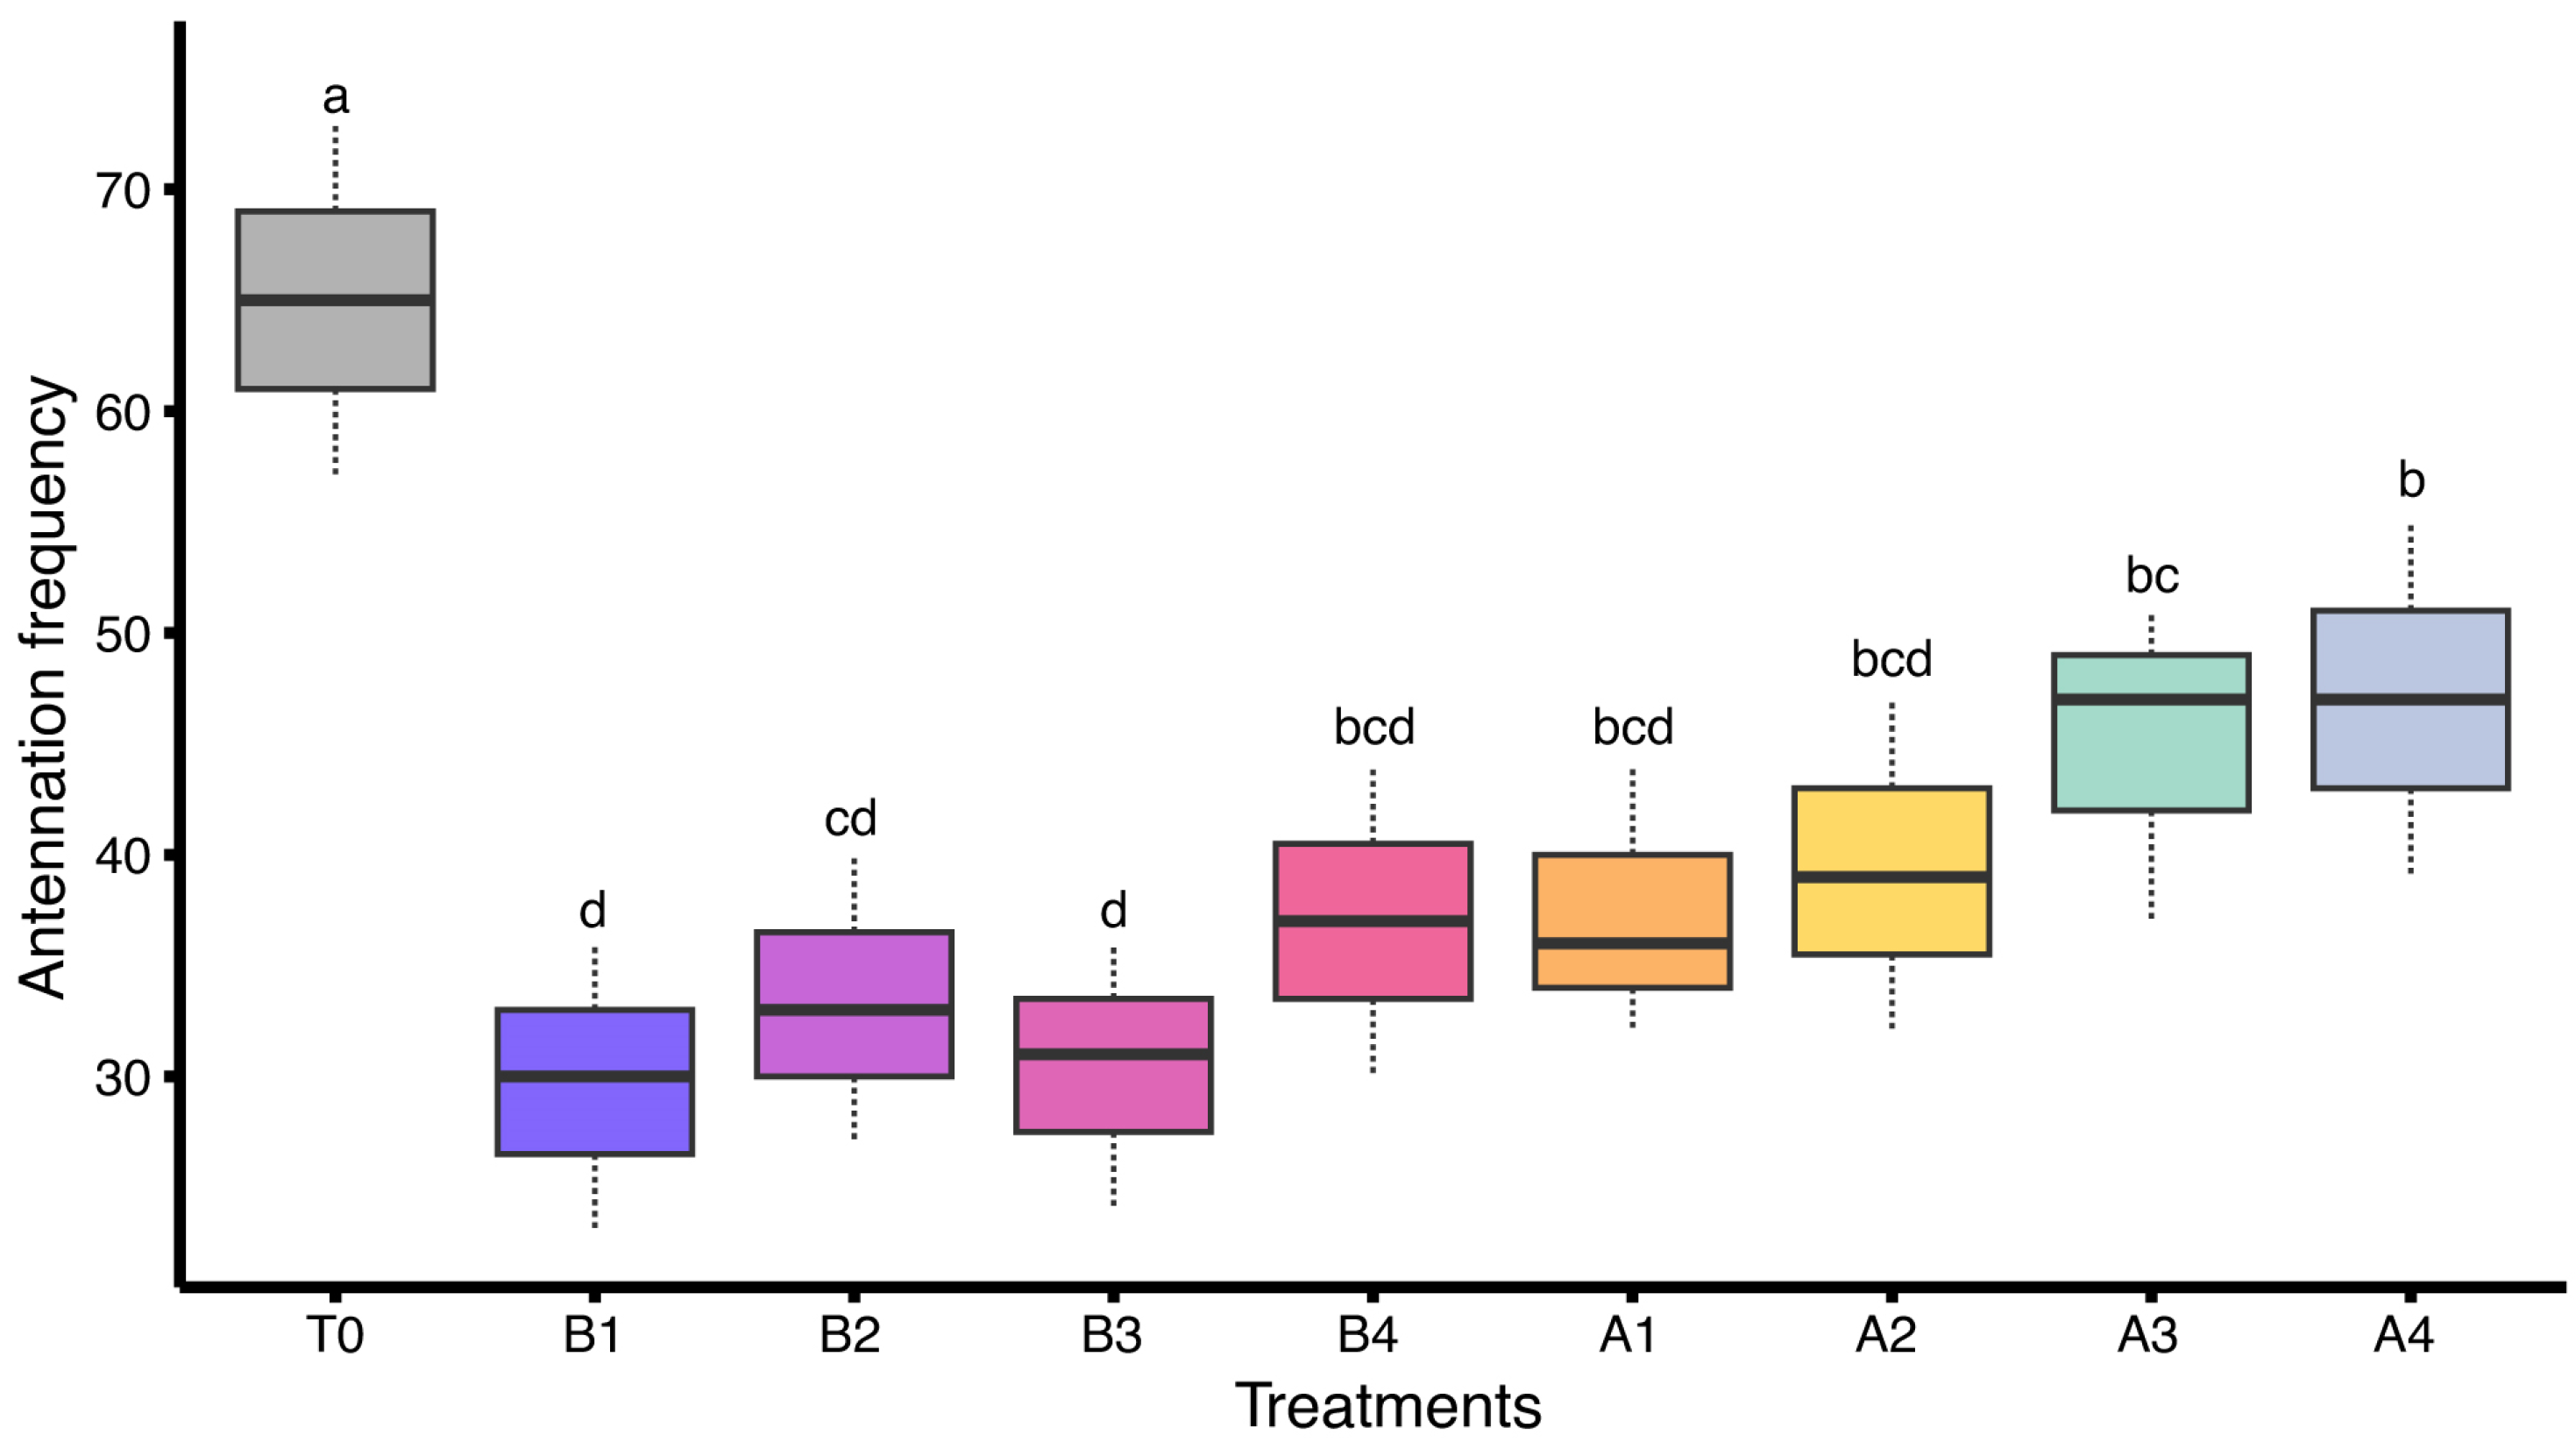
Similarly, a statistically significant difference was observed in antennation behavior of honey bee colonies subjected to various insecticide treatments under field conditions (F(8,18) = 7.29, p < 0.05). The highest frequency was recorded in the control group (T0: 65.00 ± 4.62), reflecting strong social interaction. Moderate levels were observed in A4 (47.00 ± 4.62) and A3 (45.00 ± 4.16), followed by lower activity in A2 (39.33 ± 4.33), A1 (37.33 ± 3.53), and T4 (37.00 ± 4.04). Reduced antennation was seen in B2 (33.33 ± 3.76), B3 (30.33 ± 3.48), and the lowest was observed in B1 (29.67 ± 3.76). These results support the conclusion that sub-lethal insecticide exposure reduces social responsiveness within the colony (Figure 6).
Figure 6.
Antennation frequency in honey bee colonies treated with various insecticides under field conditions (n = 3 colonies per treatment). Different letters indicate statistically significant differences among treatments based on LSD test at α = 0.05. The dashed lines (whiskers) above and below of each box represent data variability.
3.3. Pearson’s Correlation
The Pearson correlation between two critical social behaviors of A. mellifera—trophallaxis (food-sharing behavior) and antennation (antenna-based social contact)—was observed. The Pearson correlation coefficient (r = 0.94) indicated a very strong positive relationship, meaning that as trophallaxis increased, antennation also tended to increase, and vice versa. The statistical significance of this correlation was confirmed by the p-value < 0.001, indicating a highly significant association. These findings suggested that both behaviors were closely interlinked and potentially influenced by shared stressors, such as sub-lethal insecticidal exposure. Therefore, disruptions in either of these behaviors could serve as early indicators of compromised colony social dynamics under indirect insecticide stress. This highlights that both social behaviors are closely interlinked and can serve as sensitive indicators of colony stress under sub-lethal insecticidal exposure.
3.4. Longevity and Reproduction
A statistically significant difference was observed in fecundity and adult bee lifespan of honey bees belonging to colonies which were subjected to different insecticide treatments under field conditions. Fecundity varied significantly across treatments (F(8,18) = 5.6, p < 0.01), with the highest egg-laying recorded in the control group (T0: 250.00 ± 12.10), followed by A4 (214.00 ± 11.24) and A3 (203.67 ± 11.78). The lowest fecundity was observed in B1 (169.33 ± 8.37), indicating reduced reproductive output under that treatment. Similarly, adult bee lifespan differed significantly (F(8,18) = 11.0, p < 0.01), with the longest lifespan observed in T0 (41.67 ± 0.33 days), followed closely by B4 (41.33 ± 0.67) and A4 (40.67 ± 0.67). The shortest lifespans were observed in B1 and B2 (36.33 ± 0.88 and 36.33 ± 0.33 days, respectively), reflecting the weaker support provided by these treatments for bee longevity. The results further showed slight but statistically non-significant variations regarding the hatching period (F = 1.25, p = 0.3276), larval period (F = 1.29, p = 0.308), or pupal period (F = 0.85, p = 0.5705), suggesting relatively uniform developmental durations across all tested treatments during these stages. However, numerical differences were noted: A2 had the shortest larval period (5.00 ± 0.00 days), while T0 and A4 had the longest (6.00 ± 0.00 days). Similarly, the pupal period remained at 12.00 ± 0.00 days in T0 and A4, whereas slightly shorter durations were recorded in other treatments (Table 2).
Table 2.
Effects of different insecticide treatments on fecundity, hatching period, larval period, pupal period, and adult bee lifespan of Apis mellifera colonies under field conditions (n = 3 colonies per treatment). Values were expressed as mean ± SE. Different superscript letters within the same column indicate statistically significant differences among treatments based on LSD test at α = 0.05.
4. Discussion
The current study introduces a novel perspective in honey bee toxicology by examining the sub-lethal trophic (dietary) pathway of insecticidal exposure instead of conventional toxicity routes (direct and surface residual). The current research assessed the individual dietary trophic effect of bifenthrin and acetamiprid on some colony parameters such as foraging behavior, social interaction, and longevity of A. mellifera under field conditions.
The foraging activities of bees showed a consistent decline when colonies were exposed to a higher concentration of insecticides, especially bifenthrin at 1/2 (B1) and 1/4 (B2). The control group (T0) showed the best foraging activities, with the maximum number of bees returning to hives, suggesting optimal colony performance in the absence of chemical stress. The current results were supported by the findings of Henry et al. [35], who proved that application of thiamethoxam decreased the capability of the foragers to come back to the hive, which they explained might be due to the loss of navigation as a results of neurotoxic effect of applied chemical. Similarly, Decourtye et al. [58] reported that application of sub-lethal concentrations of deltamethrin and imidacloprid influenced the learning and orientation of bees, resulting in reduced foraging success. Moreover, a moderate decline in foraging activity was also observed at lower insecticide doses (B3–A4), indicating that chronic trophic exposure, even at reduced concentrations, may influence foraging efficiency over time rather than causing immediate disruption. This aligns with the work of Tosi and Nieh [59], who pointed out that flupyradifurone, another systemic insecticide, caused long-term behavioral interference in bees even at low doses. Similarly, Mustard et al. [60] reported that honey bees exposed to different pesticide-treated nectars and pollens remain confused in perceiving floral odors, which significantly compromises (up to 40%) their foraging activities. This might be attributed to the fact that pesticidal exposure alters the neural pathways linked with associative learning, making it difficult for bees to find food resources and locate earlier valuable floral sources [61]. The current results were further supported by Piiroinen and Goulson [62], who reported that chronic exposure to new-chemistry insecticides delays learning speed and cognitive processing in bumblebees and honey bees. These learning delays are mostly associated with weaker colony stability and reduced foraging activities. Moreover, the time span for recording these observations varied in different studies. but a two-hour window in the morning, as mentioned in current study, usually represents the peak foraging time interval of honey bees in different ecosystems [41,47,50,63]. Moreover, foragers possess the ability to remember the specific time of the day during which they found abundant food resources and later prefer that time to initiate their foraging activities [64]. However, the usual foraging interval at a specific feeding site is no more than five minutes [65].
The collection of pollens is a direct indicator of the performance of foraging and nutritional conditions of colonies. Bees exposed to higher concentrations of bifenthrin (B1, B2) and acetamiprid (A1) collected less pollen than the untreated control. Such declines have also been reported by Singla et al. [66], who noted that the neonicotinoids decreased the quantity of pollen on returning foragers because of motor deficiencies and reduced floral attraction. In addition, social behaviors such as trophallaxis and antennation were reduced in pesticide-treated colonies, suggesting potential disruption of intra-colony communication rather than complete behavioral suppression. Trophallaxis, essential for food sharing and pheromonal communication, was highest in T0 but decreased in proportion against the rising level of insecticide exposure, especially in B1 and B2. These findings were consistent with Murphree [67], who reported that neonicotinoids interfered with the recognition of colony mates and reduced trophallaxis frequency in pesticide exposed colonies.
Similarly, antennation behavior, which serves as a key element of colony coordination and task allocation, was severely impacted by pesticidal exposure. Palmer-Young et al. [68] reported that cholinergic pesticides may impair sensory neuron function, reducing responsiveness to social cues. In the present study, reduced antennation frequency in B1–B3 colonies suggests altered social responsiveness rather than complete loss of social function. These results are in line with our findings, which revealed significantly reduced antennation in B1-B3 colonies. These treatments also had significant effects on both fecundity and adult bee lifespan. The control group had the greatest fecundity and longevity, while B1 and B2 had a sharp decrease in these tested parameters. These findings were consistent with Wu et al. [24], who reported that bees reared on pesticide-contaminated combs had reduced lifespans. Wu-Smart and Spivak [69] also documented reduced queen fecundity and reduced worker lifespan with a long-term neonicotinoid exposure. Although no statistically significant differences were detected in hatching period, larval duration, or pupal period, slight numerical reductions in treated colonies (notably A2) may indicate subtle physiological stress rather than overt developmental failure, as proposed by Rondeau et al. [70]. Thus, these findings reinforce that the continuous exposure of sub-lethal levels of insecticides gradually affects the functional capacity of the bee colonies.
5. Conclusions
Conclusively, it is stated that current experiments conducted under apiary field conditions might be influenced by unavoidable environmental stressors that cannot be fully controlled. However, field conditions were intentionally selected to reflect realistic exposure scenarios to enhance the ecological relevance of the findings. The current experiments demonstrate that the trophic exposure via contaminated diet to sub-lethal doses of bifenthrin and acetamiprid negatively influences the key colony performance traits of A. mellifera, including foraging activity, social behavior, and longevity, in a dose-dependent manner. Higher concentrations (B1, B2, A1, A2) caused more pronounced behavioral and survival impairments, whereas the lower doses (A3, A4) produced moderate effects. Reduced foraging, fewer outgoing/returning bees, and reduced pollen collection were indications of impaired orientation, likely due to neurotoxic effects. Reductions in trophallaxis and antennation further suggested impaired social feeding and social integration. Drastic declines in fecundity and adult longevity also reflected physiological stress, and small changes in brood development may indicate more subtle developmental effects. Overall, the outcomes of this study emphasized that the prolonged ingestion of pesticide-contaminated food, even at sub-lethal levels, can gradually disrupt fundamental colony functions and social stability. This underlines the critical need to consider trophic pesticidal exposure pathways in pollinator risk evaluations. This is particularly concerning for agro-ecosystems reliant on pollination, as continued pesticide exposure may jeopardize the long-term sustainability of A. mellifera populations and their ecological services. Therefore, future studies should focus on integrating molecular and physiological biomarkers to link behavioral changes with underlying mechanisms, validating pollen sources collected by foragers through palynological analysis, expanding experiments to multiple crops and regions, evaluating pesticide mixtures and field-relevant exposure scenarios, and employing automated or longer-term behavioral monitoring to reduce subjectivity. Long-term field trials conducted over several seasons are also recommended to better understand chronic and cumulative effects.
Author Contributions
Conceptualization, M.U.Y., M.A.A., S.U.I. and S.A.; methodology, M.U.Y., S.U.I., R.A. and M.S. (Muhammad Saqib); software, S.U.I., M.S. (Muhammad Saqib), M.S. (Mishal Subhan), S.A., M.N.S. and A.H.; validation, M.A.A., S.A., N.J.K. and A.H.; formal analysis, M.U.Y., M.N.S., N.J.K., A.H., S.U.I. and M.S. (Muhammad Saqib); investigation, M.U.Y., S.A., N.J.K. and R.A.; resources, M.A.A., S.A., R.A. and S.U.I.; data curation, M.U.Y., M.N.S., A.H., M.S. (Mishal Subhan), M.S. (Muhammad Saqib) and S.U.I.; writing—original draft preparation, M.U.Y., M.A.A., S.U.I. and A.H.; writing—review and editing, S.A., R.A., M.S. (Mishal Subhan), M.S. (Muhammad Saqib) and N.J.K.; visualization, M.A.A. and S.A.; supervision, M.A.A.; project administration, M.U.Y. and M.A.A.; funding acquisition, A.H., M.S. (Mishal Subhan) and M.N.S. All authors have read and agreed to the published version of the manuscript.
Funding
The authors extend their appreciation to The Higher Education Commission of Pakistan for supporting this work through project number (NRPU/20/15650) and ORIC, IUB for facilitation under project number (3905/ORIC/IUB/2021).
Data Availability Statement
The original contributions presented in this study are included in the article. Further inquiries can be directed to the corresponding authors.
Conflicts of Interest
The authors declare that they have no known competing financial interests or personal relationships that could have appeared to influence the work reported in this paper.
References
- Ahsan, Z.; Wu, Z.; Lin, Z.; Ji, T.; Wang, K. The Sublethal Effects of Neonicotinoids on Honeybees. Biology 2025, 14, 1076. [Google Scholar] [CrossRef] [Scilit]
- Papa, G.; Maier, R.; Durazzo, A.; Lucarini, M.; Karabagias, I.K.; Plutino, M.; Bianchetto, E.; Aromolo, R.; Pignatti, G.; Ambrogio, A.; et al. The honey bee Apis mellifera: An insect at the interface between human and ecosystem health. Biology 2022, 11, 233. [Google Scholar] [CrossRef] [Scilit]
- Klein, A.-M.; Vaissière, B.E.; Cane, J.H.; Steffan-Dewenter, I.; Cunningham, S.A.; Kremen, C.; Tscharntke, T. Importance of pollinators in changing landscapes for world crops. Proc. R. Soc. B Biol. Sci. 2007, 274, 303–313. [Google Scholar] [CrossRef] [Scilit]
- Calderone, N.W. Insect pollinated crops, insect pollinators and US agriculture: Trend analysis of aggregate data for the period 1992–2009. PLoS ONE 2012, 7, e37235. [Google Scholar] [CrossRef] [Scilit]
- Seeley, T.D. The Wisdom of the Hive: The Social Physiology of Honey Bee Colonies; Harvard University Press: Cambridge, MA, USA, 2009. [Google Scholar]
- Goulson, D.; Nicholls, E.; Botías, C.; Rotheray, E.L. Bee declines driven by combined stress from parasites, pesticides, and lack of flowers. Science 2015, 347, 1255957. [Google Scholar] [CrossRef] [Scilit]
- Straub, L.; Villamar-Bouza, L.; Bruckner, S.; Chantawannakul, P.; Kolari, E.; Maitip, J.; Vidondo, B.; Neumann, P.; Williams, G.R. Negative effects of neonicotinoids on male honeybee survival, behaviour and physiology in the field. J. Appl. Ecol. 2021, 58, 2515–2528. [Google Scholar] [CrossRef] [Scilit]
- Hendriksma, H.P.; Toth, A.L.; Shafir, S. Individual and colony level foraging decisions of bumble bees and honey bees in relation to balancing of nutrient needs. Front. Ecol. Evol. 2019, 7, 177. [Google Scholar] [CrossRef] [Scilit]
- Conte, Y.L.; Hefetz, A. Primer pheromones in social hymenoptera. Annu. Rev. Entomol. 2008, 53, 523–542. [Google Scholar] [CrossRef] [Scilit]
- Moreira, D.R.; de Souza, T.H.S.; Galhardo, D.; Figueira, C.L.; Baulli, S.C.; da Silva, B.G.; das Chagas, F.; Oliveira, J.W.S.; Rocha, J.S.; de Souza Khatlab, A.; et al. Exposure of Apis mellifera (Hymenoptera: Apidae) colonies to imidacloprid impairs larval development, promotes oxidative stress in pupae, and induces changes in the midgut of adult bees. Biol. Res. 2025, 58, 5. [Google Scholar] [CrossRef] [Scilit]
- Potts, S.G.; Roberts, S.P.; Dean, R.; Marris, G.; Brown, M.A.; Jones, R.; Neumann, P.; Settele, J. Declines of managed honey bees and beekeepers in Europe. J. Apic. Res. 2010, 49, 15–22. [Google Scholar] [CrossRef] [Scilit]
- Diao, Q.; Li, B.; Zhao, H.; Wu, Y.; Guo, R.; Dai, P.; Chen, D.; Wang, Q.; Hou, C. Enhancement of chronic bee paralysis virus levels in honeybees acute exposed to imidacloprid: A Chinese case study. Sci. Total Environ. 2018, 630, 487–494. [Google Scholar] [CrossRef] [Scilit]
- Tosi, S.; Costa, C.; Vesco, U.; Quaglia, G.; Guido, G. A 3-year survey of Italian honey bee-collected pollen reveals widespread contamination by agricultural pesticides. Sci. Total Environ. 2018, 615, 208–218. [Google Scholar] [CrossRef] [Scilit]
- Sanchez-Bayo, F.; Goka, K. Pesticide residues and bees–a risk assessment. PLoS ONE 2014, 9, e94482. [Google Scholar] [CrossRef] [Scilit]
- Sukkar, D.; Wagner, L.; Bonnefoy, A.; Falla-Angel, J.; Laval-Gilly, P. Diverse alterations and correlations in antioxidant gene expression in honeybee (Apis mellifera) hemocytes interacting with microbial pathogen-associated molecular patterns and pesticide cocktails. Environ. Toxicol. Pharmacol. 2025, 114, 104649. [Google Scholar] [CrossRef] [Scilit]
- Di Noi, A.; Casini, S.; Campani, T.; Cai, G.; Caliani, I. Review on sublethal effects of environmental contaminants in honey bees (Apis mellifera), knowledge gaps and future perspectives. Int. J. Environ. Res. Public Health 2021, 18, 1863. [Google Scholar] [CrossRef] [Scilit]
- Pereira, N.; Diniz, T.; Takasusuki, M. Sublethal effects of neonicotinoids in bees: A review. Sci. Electron. Arch. 2020, 13, 142–152. [Google Scholar] [CrossRef] [Scilit]
- Zuščíková, L.; Bažány, D.; Greifová, H.; Knížatová, N.; Kováčik, A.; Lukáč, N.; Jambor, T. Screening of toxic effects of neonicotinoid insecticides with a focus on acetamiprid: A review. Toxics 2023, 11, 598. [Google Scholar] [CrossRef] [Scilit]
- Abuagla, M.I.; Iqbal, J.; Raweh, H.S.; Alqarni, A.S. Insight into olfactory learning, memory, and mortality of Apis mellifera jemenitica after exposure to acetamiprid insecticide. Insects 2024, 15, 473. [Google Scholar] [CrossRef] [Scilit]
- Wang, Y.; Zhu, Y.C.; Li, W. Interaction patterns and combined toxic effects of acetamiprid in combination with seven pesticides on honey bee (Apis mellifera L.). Ecotoxicol. Environ. Saf. 2020, 190, 110100. [Google Scholar] [CrossRef] [Scilit]
- Williamson, S.M.; Willis, S.J.; Wright, G.A. Exposure to neonicotinoids influences the motor function of adult worker honeybees. Ecotoxicology 2014, 23, 1409–1418. [Google Scholar] [CrossRef] [Scilit]
- Milone, J.P.; Tarpy, D.R. Effects of developmental exposure to pesticides in wax and pollen on honey bee (Apis mellifera) queen reproductive phenotypes. Sci. Rep. 2021, 11, 1020. [Google Scholar] [CrossRef] [Scilit]
- Mullin, C.A. Effects of ‘inactive’ingredients on bees. Curr. Opin. Insect Sci. 2015, 10, 194–200. [Google Scholar] [CrossRef] [Scilit]
- Wu, J.Y.; Anelli, C.M.; Sheppard, W.S. Sub-lethal effects of pesticide residues in brood comb on worker honey bee (Apis mellifera) development and longevity. PLoS ONE 2011, 6, e14720. [Google Scholar] [CrossRef] [Scilit]
- Ben Abdelkader, F.; Çakmak, İ.; Çakmak, S.S.; Nur, Z.; İncebıyık, E.; Aktar, A.; Erdost, H. Toxicity assessment of chronic exposure to common insecticides and bee medications on colony development and drones sperm parameters. Ecotoxicology 2021, 30, 806–817. [Google Scholar] [CrossRef] [Scilit]
- Desneux, N.; Decourtye, A.; Delpuech, J.-M. The sublethal effects of pesticides on beneficial arthropods. Annu. Rev. Entomol. 2007, 52, 81–106. [Google Scholar] [CrossRef] [Scilit]
- Aqueel, M.A.; Shurjeel, H.K.; Ali, S.; Bakar, M.A.; Sohail, M.; Qadir, Z.A.; Manzoor, A. Natural foraging and artificial feeding of domesticated honeybees. Adv. Insect Pollinat. Technol. Sustain. Agric. 2023, 3, 234. [Google Scholar]
- Williamson, S.M.; Baker, D.D.; Wright, G.A. Acute exposure to a sublethal dose of imidacloprid and coumaphos enhances olfactory learning and memory in the honeybee Apis mellifera. Invertebr. Neurosci. 2013, 13, 63–70. [Google Scholar] [CrossRef] [Scilit]
- Brandt, A.; Gorenflo, A.; Siede, R.; Meixner, M.; Büchler, R. The neonicotinoids thiacloprid, imidacloprid, and clothianidin affect the immunocompetence of honey bees (Apis mellifera L.). J. Insect Physiol. 2016, 86, 40–47. [Google Scholar] [CrossRef] [Scilit]
- Trhlin, M.; Rajchard, J. Chemical communication in the honeybee (Apis mellifera L.): A review. Vet. Med. 2011, 56, 265–273. [Google Scholar] [CrossRef] [Scilit]
- Pettis, J.S.; Rice, N.; Joselow, K.; vanEngelsdorp, D.; Chaimanee, V. Colony failure linked to low sperm viability in honey bee (Apis mellifera) queens and an exploration of potential causative factors. PLoS ONE 2016, 11, e0147220. [Google Scholar]
- Morfin, N.; Goodwin, P.H.; Correa-Benitez, A.; Guzman-Novoa, E. Sublethal exposure to clothianidin during the larval stage causes long-term impairment of hygienic and foraging behaviours of honey bees. Apidologie 2019, 50, 595–605. [Google Scholar] [CrossRef] [Scilit]
- Pamminger, T.; Basley, K.; Goulson, D.; Hughes, W.O. Potential acetylcholine-based communication in honeybee haemocytes and its modulation by a neonicotinoid insecticide. PeerJ 2024, 12, e17978. [Google Scholar] [CrossRef] [Scilit]
- Collison, E.J.; Hird, H.; Tyler, C.R.; Cresswell, J.E. Effects of neonicotinoid exposure on molecular and physiological indicators of honey bee immunocompetence. Apidologie 2018, 49, 196–208. [Google Scholar] [CrossRef] [Scilit]
- Henry, M.; Beguin, M.; Requier, F.; Rollin, O.; Odoux, J.-F.; Aupinel, P.; Aptel, J.; Tchamitchian, S.; Decourtye, A. A common pesticide decreases foraging success and survival in honey bees. Science 2012, 336, 348–350. [Google Scholar] [CrossRef] [Scilit]
- Naug, D. Nutritional stress due to habitat loss may explain recent honeybee colony collapses. Biol. Conserv. 2009, 142, 2369–2372. [Google Scholar] [CrossRef] [Scilit]
- Sihag, R.C.; Rawal, G.K. Effect of initial colony strength on productivity and pollination services of honey bee (Apis mellifera L.). EUREKA Life Sci. 2025, 1, 19–28. [Google Scholar] [CrossRef] [Scilit]
- Gill, R.J.; Ramos-Rodriguez, O.; Raine, N.E. Combined pesticide exposure severely affects individual-and colony-level traits in bees. Nature 2012, 491, 105–108. [Google Scholar] [CrossRef] [Scilit]
- Islam, S.U.; Aqueel, M.A.; Yousuf, M.U.; Abbasi, A.; Yasin, M.; Iqbal, R.; Raza, M.F.; Parvaiz, A.; Rebouh, N.Y. Evaluating the Influence of Different Artificial Diets on Apis mellifera L. Using Health Biomarkers and Performance Metrics. Insects 2024, 15, 905. [Google Scholar] [CrossRef] [Scilit]
- Shurjeel, H.K.; Aqueel, M.A.; Ashraf, E.; Ali, A.; Rubab, A. Effect of insecticides on the longevity of Apis mellifera L. (Hymenoptera: Apidae). Sarhad J. Agric. 2020, 36, 768–776. [Google Scholar] [CrossRef] [Scilit]
- Abou-Shaara, H.F. The foraging behaviour of honey bees, Apis mellifera: A review. Vet. Med. 2014, 59, 1–10. [Google Scholar]
- Rutschmann, B.; Kohl, P.L.; Steffan-Dewenter, I. Foraging distances, habitat preferences and seasonal colony performance of honeybees in Central European forest landscapes. J. Appl. Ecol. 2023, 60, 1056–1066. [Google Scholar] [CrossRef] [Scilit]
- Gulati, R.; Kumari, B.; Sharma, S. Field residual toxicity of some insecticides to honeybee (Apis mellifera L.) and residues of common insecticides from apiary honey. J. Apic. 2004, 19, 51–56. [Google Scholar]
- Ji, J.-Y.; Yang, J.; Zhang, B.-W.; Wang, S.-R.; Zhang, G.-C.; Lin, L.-N. Sodium pheophorbide a controls cherry tomato gray mold (Botrytis cinerea) by destroying fungal cell structure and enhancing disease resistance-related enzyme activities in fruit. Pestic. Biochem. Physiol. 2020, 166, 104581. [Google Scholar] [CrossRef] [Scilit]
- Horne, M. Knapsack sprayers: Operators, standards and selection. Outlooks Pest Manag. 2019, 30, 171–175. [Google Scholar] [CrossRef] [Scilit]
- Beekman, M.; Nederstigt, C.; Suchiman, H.E.D.; Kremer, D.; van der Breggen, R.; Lakenberg, N.; Alemayehu, W.G.; de Craen, A.J.; Westendorp, R.G.; Boomsma, D.I.; et al. Genome-wide association study (GWAS)-identified disease risk alleles do not compromise human longevity. Proc. Natl. Acad. Sci. USA 2010, 107, 18046–18049. [Google Scholar] [CrossRef] [Scilit]
- Alqarni, A.S. Tolerance of summer temperature in imported and indigenous honeybee Apis mellifera L. races in central Saudi Arabia. Saudi J. Biol. Sci. 2006, 13, 123–127. [Google Scholar]
- Pernal, S.F.; Currie, R.W. The influence of pollen quality on foraging behavior in honeybees (Apis mellifera L.). Behav. Ecol. Sociobiol. 2001, 51, 53–68. [Google Scholar] [CrossRef] [Scilit]
- Manzoor, A.; Aqueel, M.A.; Islam, S.U.; Dessoky, E.S.; Ahsan, M.H.; Ahmad, B.; Yousuf, M.U.; Saqib, M.; Raza, M.F.; Iqbal, R. Assessment of consumption and digestibility of artificial diets and their effects on few life study parameters of Apis mellifera L. Asian J. Agric. Biol. 2025, 1, 2024105. [Google Scholar] [CrossRef] [Scilit]
- Joshi, N.C.; Joshi, P. Foraging behaviour of Apis spp. on apple flowers in a subtropical environment. N. Y. Sci. J. 2010, 3, 71–76. [Google Scholar]
- Goyret, J.; Farina, W. Descriptive study of antennation during trophallactic unloading contacts in honeybees Apis mellifera carnica. Insectes Sociaux 2003, 50, 274–276. [Google Scholar] [CrossRef] [Scilit]
- Wright, G.A.; Lillvis, J.L.; Bray, H.J.; Mustard, J.A. Physiological state influences the social interactions of two honeybee nest mates. PLoS ONE 2012, 7, e32677. [Google Scholar] [CrossRef] [Scilit]
- Boff, S.; Friedel, A.; Mussury, R.M.; Lenis, P.R.; Raizer, J. Changes in social behavior are induced by pesticide ingestion in a Neotropical stingless bee. Ecotoxicol. Environ. Saf. 2018, 164, 548–553. [Google Scholar] [CrossRef] [Scilit]
- Forfert, N.; Moritz, R.F. Thiacloprid alters social interactions among honey bee workers (Apis mellifera). J. Apic. Res. 2017, 56, 467–474. [Google Scholar] [CrossRef] [Scilit]
- Woyke, J. Brood-rearing efficiency and absconding in Indian honeybees. J. Apic. Res. 1976, 15, 133–143. [Google Scholar] [CrossRef] [Scilit]
- Islam, S.U.; Liaquat, J.; Aqueel, M.A.; Abbasi, A.; Arshad, M.; Rizwan, M.S.; Saqib, M.; Masood, N.; Kavhiza, N.J.; Zafar, S.; et al. Effect of Diet Compositions on Colony Strength Parameters, and the Enzymatic Activity of Apis mellifera L. During Floral Scarcity. Insects 2025, 16, 967. [Google Scholar] [CrossRef] [Scilit]
- Martin, S.J.; Hawkins, G.P.; Brettell, L.E.; Reece, N.; Correia-Oliveira, M.E.; Allsopp, M.H. Varroa destructor reproduction and cell re-capping in mite-resistant Apis mellifera populations. Apidologie 2020, 51, 369–381. [Google Scholar] [CrossRef] [Scilit]
- Decourtye, A.; Armengaud, C.; Renou, M.; Devillers, J.; Cluzeau, S.; Gauthier, M.; Pham-Delègue, M.-H. Imidacloprid impairs memory and brain metabolism in the honeybee (Apis mellifera L.). Pestic. Biochem. Physiol. 2004, 78, 83–92. [Google Scholar] [CrossRef] [Scilit]
- Tosi, S.; Nieh, J. Lethal and sublethal synergistic effects of a new systemic pesticide, flupyradifurone (Sivanto®), on honeybees. Proc. R. Soc. B 2019, 286, 20190433. [Google Scholar]
- Mustard, J.A.; Gott, A.; Scott, J.; Chavarria, N.L.; Wright, G.A. Honeybees fail to discriminate floral scents in a complex learning task after consuming a neonicotinoid pesticide. J. Exp. Biol. 2020, 223, jeb217174. [Google Scholar] [CrossRef] [Scilit]
- Siviter, H.; Koricheva, J.; Brown, M.J.; Leadbeater, E. Quantifying the impact of pesticides on learning and memory in bees. J. Appl. Ecol. 2018, 55, 2812–2821. [Google Scholar] [CrossRef] [Scilit]
- Piiroinen, S.; Goulson, D. Chronic neonicotinoid pesticide exposure and parasite stress differentially affects learning in honeybees and bumblebees. Proc. R. Soc. B Biol. Sci. 2016, 283, 20160246. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Reyes-Carrillo, J.L.; Eischen, F.A.; Cano-Rios, P.; Rodriguez-Martinez, R.; Nava Camberos, U. Pollen collection and honey bee forager distribution in cantaloupe. Acta Zool. Mex. 2007, 23, 29–36. [Google Scholar] [CrossRef] [Scilit]
- Silva, D.P.; Moisan-De Serres, J.; Souza, D.R.; Hilgert-Moreira, S.B.; Fernandes, M.Z.; Kevan, P.G.; Freitas, B.M. Efficiency in pollen foraging by honey bees: Time, motion and pollen depletion on flowers of Sisyrinchium palmifolium Linnaeus (Asparagales: Iridaceae). J. Pollinat. Ecol. 2013, 11, 27–32. [Google Scholar] [CrossRef] [Scilit]
- Yang, E.; Chuang, Y.C.; Chen, Y.; Chang, L. Abnormal foraging behavior induced by sublethal dosage of imidacloprid in the honey bee (Hymenoptera: Apidae). J. Econ. Entomol. 2008, 101, 1743–1748. [Google Scholar] [CrossRef] [Scilit]
- Singla, A.; Barmota, H.; Kumar Sahoo, S.; Kaur Kang, B. Influence of neonicotinoids on pollinators: A review. J. Apic. Res. 2021, 60, 19–32. [Google Scholar] [CrossRef] [Scilit]
- Murphree, S.M. Effects of Imidacloprid and Octopamine on the Honey Bee (Apis mellifera) Trophallaxis Social Network. Master’s Thesis, University of Illinois at Urbana-Champaign, Champaign, IL, USA, 2022. [Google Scholar]
- Palmer-Young, E.C.; Tozkar, C.Ö.; Schwarz, R.S.; Chen, Y.; Irwin, R.E.; Adler, L.S.; Evans, J.D. Nectar and pollen phytochemicals stimulate honey bee (Hymenoptera: Apidae) immunity to viral infection. J. Econ. Entomol. 2017, 110, 1959–1972. [Google Scholar] [CrossRef] [Scilit]
- Wu-Smart, J.; Spivak, M. Sub-lethal effects of dietary neonicotinoid insecticide exposure on honey bee queen fecundity and colony development. Sci. Rep. 2016, 6, 32108. [Google Scholar] [CrossRef] [Scilit]
- Rondeau, N.C.; Raup-Collado, J.; Kogan, H.V.; Cho, R.; Lovinger, N.; Wague, F.; Lopatkin, A.J.; Texeira, N.G.; Flores, M.E.; Rovnyak, D.; et al. Remodeling of Cellular Respiration and Insulin Signaling Are Part of a Shared Stress Response in Divergent Bee Species. Insects 2025, 16, 300. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.