


Abstract
Hydraulic redistribution (HR) in plants facilitates bidirectional water transport through the vascular system in response to soil water potential gradients, with implications for ecological facilitation. This study aimed to evaluate the efficacy and results obtained with high-precision weighing lysimeters in detecting HR in olive (Olea europaea L.) using a split-root experimental setup with potted trees. Sixteen pots, each containing half of a plant’s root system, were independently monitored for mass changes to quantify HR between irrigated and water-stressed compartments. The independent weighing of each pair of linked pots was a challenge, but the purpose-built precision lysimeter array effectively isolated weights despite mechanical connections between pot pairs. Results demonstrated measurable water redistribution via roots from irrigated to dry pots, with mass transfer from the irrigated side to the non-irrigated side of the plants, between 10 and 70 g. After irrigation, non-irrigated pots received by HR on average between 3 and 12% of the irrigation water applied in irrigated pots. This furthermore highlighted the potential of the lysimeters for precise quantification of plant-mediated water dynamics. It was observed that HR intensity peaked shortly after irrigation, some hours to one day, and diminished over time, with higher intensity during nocturnal periods or cloudy humid daily conditions of negligible or null evapotranspiration. These findings confirm previous observations with reverse sap flow sensors, now with a different experimental approach, which appears precise but only possible for potted plants, allowing further understanding of HR.
1. Introduction
There is extensive experimental evidence [1,2] that deep-rooted plants can transport water from deep soil or groundwater to roots in the superficial layers, or vice versa. This occurs in response to water-potential gradients—that is, using the same bidirectional hydraulic mechanism operating in the soil–root complex, but with much less resistance. This mechanism is usually called hydraulic redistribution (HR). It has also been demonstrated (e.g., using chemical tracers) that water can be transported from superficial roots to the surrounding soil and other plants, via a process whose consequences have been discussed as ecological facilitation [2,3,4,5,6]. The importance of this mechanism and its practical implications for society has been discussed by Alagele et al. [7].
In climates with rainy winters but hot, dry summers (Mediterranean-type climates, e.g., Csa or Csb Köppen classes), the lowest water potential during the day occurs normally in the atmosphere. But, at night, the lowest potential is commonly found in the uppermost soil layers. In these climates, deep-rooted plants—which are more resilient to summer drought—can access water in deeper layers. However, during very wet and rainy winters, it is energetically advantageous for plants to exploit water in the superficial layers, where nutrients are also more abundant (e.g., [2]). This requires keeping those superficial roots alive throughout the summer dry period. In the case of nocturnal HR, the passive water is transported through the plant from deeper zones with more favorable water potential (closer to zero) to superficial zones with much lower potential. This water not only keeps the superficial root system functional. It supports some daytime transpiration from those superficial roots, thereby serving as a vehicle for nutrients present in the upper soil layers.
Consequently, in late summer, superficial roots can exhibit water flow in opposite directions with a circadian oscillation. Schematically, this oscillation can be described as follows: (1) at night: negative flow (receiving water from deep roots), direction plant → soil; (2) during the day (or part of the day): opposite direction (positive flow), soil → shoot. However, this dynamic, which reaches its greatest expression at the end of the summer dry season, can be reversed at the beginning of the rainy season. Observations on a bigger scale, and for large groups of plants, were made by several authors [8,9,10]. The analysis across climates by Quijano et al. [9] suggests that the higher rates of HR occur in Mediterranean climates.
A pioneering study in cork oak trees (Quercus suber) (2002–2003) [11] and a later two on olive orchards (Olea europaea) (2010–2012, one intensive and irrigated, the other traditional and rain-fed), employing bidirectional sap flow sensors within root systems, alongside complementary methodologies [12,13,14], elucidated the importance and dynamics of this adaptative mechanism in coping with conditions of pronounced water deficit.
Apparently, superficial roots showed the highest flow densities after rainfall periods, whereas in summer they recorded low or even negative values during much of the day. In contrast, roots shown to grow downward exhibited low flow densities during the winter rainy season and comparatively high densities during periods of water scarcity. HR was observed even in the deficit-irrigated drip-irrigated olive orchard—albeit discreetly—between roots along the irrigated row and roots that spread transversely into the inter-row space (unpublished data, Ferreira), as observed also by other authors (e.g., [2]).
The methods used were (1) the temperature-field deformation technique [15,16,17], which allows observation of bidirectional flows, providing relevant qualitative information, and (2) an alternative technique, with greater quantification capacity, the calibrated average-gradient (CAG) heat-pulse method [18,19], where a narrower averaging window for signal analysis was used to achieve a more linear calibration curve (Ferreira et al. (2018)). Although some subtle aspects of data processing can lead to nuances (CAGALG, [20]), the mechanism was fully confirmed in its daily and seasonal dynamics. It was consistent with meteorologically derived outcome conditions, as well as with soil and plant water status presented in previous publications [14]. Reverse (negative) flow was observed during about 30% of summer nights. It increased to about 5% of total daily root flow before the first autumn rains and accounting, on average, for 2.6% of total daily root flow [12].
Considering the overall study, it is possible to say that the plant survival strategy in the face of water scarcity is likely to be better explained by an increase in water uptake capacities than by a reduction in water use [21].
The HR mechanisms are especially important in regions with strong contrasts between water availability in periods of intense precipitation (orographic/Atlantic influence) and periods of extreme scarcity (summer). In Lisbon, for example, only around 5% of annual precipitation occurs in summer. Portugal is a paradigmatic case in this regard, being one of the European countries with the greatest contrast between water availability and water demand. In general, it should be emphasized that forest, agroforestry (e.g., cork oak Quercus suber, holm oak Quercus rotundifolia), and traditional non-irrigated agricultural systems such as olive (Olea europaea), grapevine (Vitis vinifera), and various other minor crops occupy vast areas of the territory in Mediterranean ecosystems of high environmental value, representative of southwestern Europe. In non-irrigated woody plants, natural deep rooting ensures survival, but maintaining synergy between the superficial and deep root systems makes plants relatively independent of rainfall patterns. This synergy can extend to associated herbaceous species, as referred to above and shown for olive [22]. This is relevant for the understanding of water use by mixed stands, where trees and herbaceous species share the same space, as in landscaping areas. Improving the knowledge on water redistribution in olive trees can inform irrigation practices, such as partial root-zone drying and regulated deficit irrigation, which involve alternating watering between different root zones to enhance water stress resilience [23].
HR has been studied with sap flow and isotope approaches and, for all methods, the aim is to measure or detect HR, but they differ in principles, invasiveness, scalability, and precision. Sap flow techniques directly measure water velocity and direction in roots or stems using thermal probes inserted into plant tissues, detecting reverse flow as evidence of HR. Isotope approaches use stable water isotopes as tracers, labeling water in one soil zone and sampling plant xylem or soil to quantify uptake and redistribution via mixing models that compare isotopic signatures to potential sources [10]. However, so far, there has been no quantification of mass transfer, i.e., the quantification of absolute mass transfer via the reference method, therefore outcoming the information provided by sap flow or isotope methods.
Conversely, past experiments with split-root systems have shown that plants can maintain growth and physiological functions even when only part of the root system is watered. In these setups, one half of the root system receives full watering while the other half receives partial watering, demonstrating stress responses [24].
To our best knowledge, no studies have addressed HR using precision mass balances combined with a split-root facility; this seemed to be the first time an attempt was made to address HR, through a split-root system linked to weighing lysimeters.
In conclusion, the primary objective of this study was to determine whether an array of high-precision lysimeters can detect and quantify root-mediated water redistribution in olive trees. To this end, an experimental system was established using potted trees configured with a split-root design. This approach enabled (i) the direct, absolute quantification of mass transfer of water between roots and (ii) a detailed temporal analysis of the dynamics of the hydraulic redistribution process.
2. Materials and Methods
2.1. Study Location and Plants’ Characterization and Preparation
The experiments were developed in a greenhouse at Instituto Superior de Agronomia, the University of Lisbon, Portugal (38°42′28.18″ N, 9°11′7.5″ W).
In March 2019, eight young olive trees (Olea europaea cv. Cobrançosa) were acquired, selected for their uniform vigor and compact size, which allowed the installation of precision weighing lysimeters with a split-root system.
The plants’ trunk diameter was approximately 10 mm. Average leaf area (LA) per plant was estimated to be 0.3 m2 by both counting the leaves (750 leaves per tree) and relating the stem diameter with leaf area, using the allometric relationships studied by [25]. This procedure yielded an area of 0.3 m2 per tree.
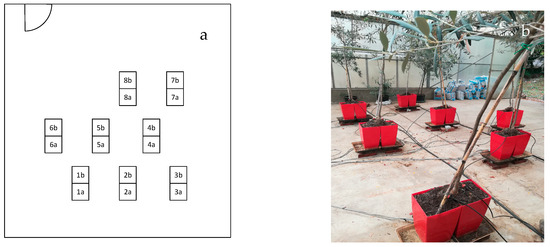
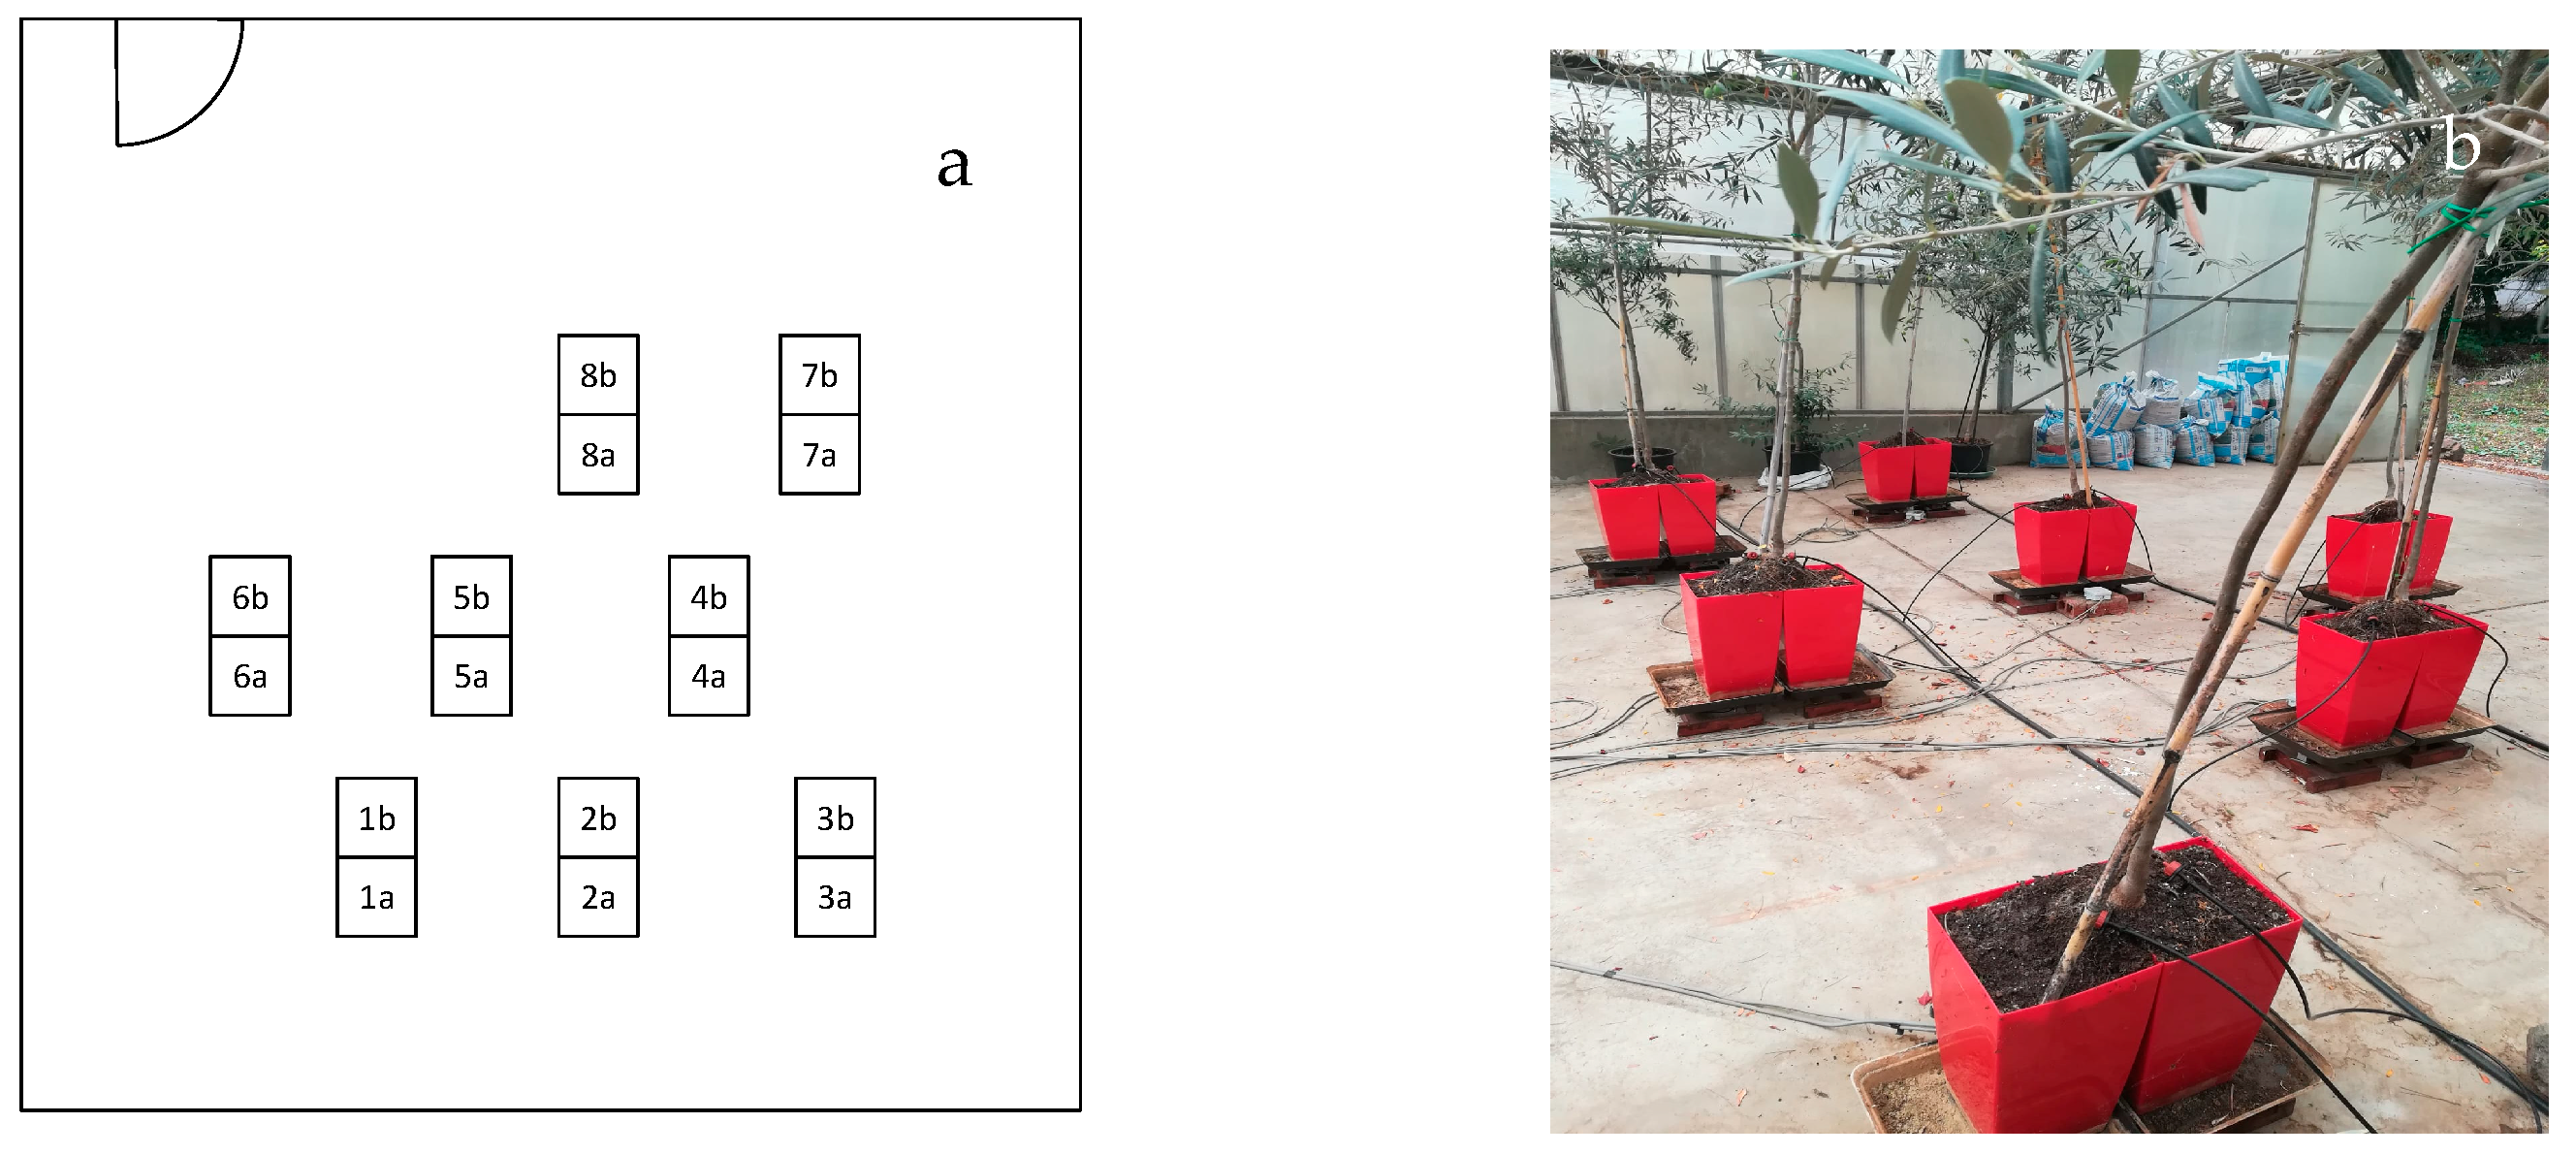
The root system of each plant was divided between two pots (A and B, Figure 1a,b) filled with a commercial substrate. A total of 16 pots (8 plants × 2 pots per plant) were used for all data analysis, except for the data collected on 30th October, where only 7 plants were used, as data provided by one pair of pots were very unstable and erroneous, which can possibly be attributed to mechanical instability of the wood frame. Pot dimensions were 35 cm width and 35 cm height (approx. 25 L volume), and the pots were randomly distributed in the greenhouse (Figure 1).
Figure 1.
Schematic view of the experimental layout (a, left) and a photo of the overall experiment (b, right) with the 8 potted olive trees in 16 pots at the greenhouse, Lisbon, Portugal.
This root-splitting operation was carried out at the beginning of the vegetative growth period (March) so that the plants could fully re-establish by October—a stage of the cycle considered suitable for conducting the trial in this species. Root regrowth occurred from the beginning of the pot’s installation.
Each pot was installed on a platform, which in turn was positioned above load cells.
2.2. Climate Characterization or Environmental Conditions During the Experiment
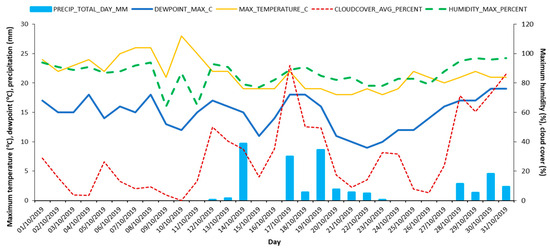
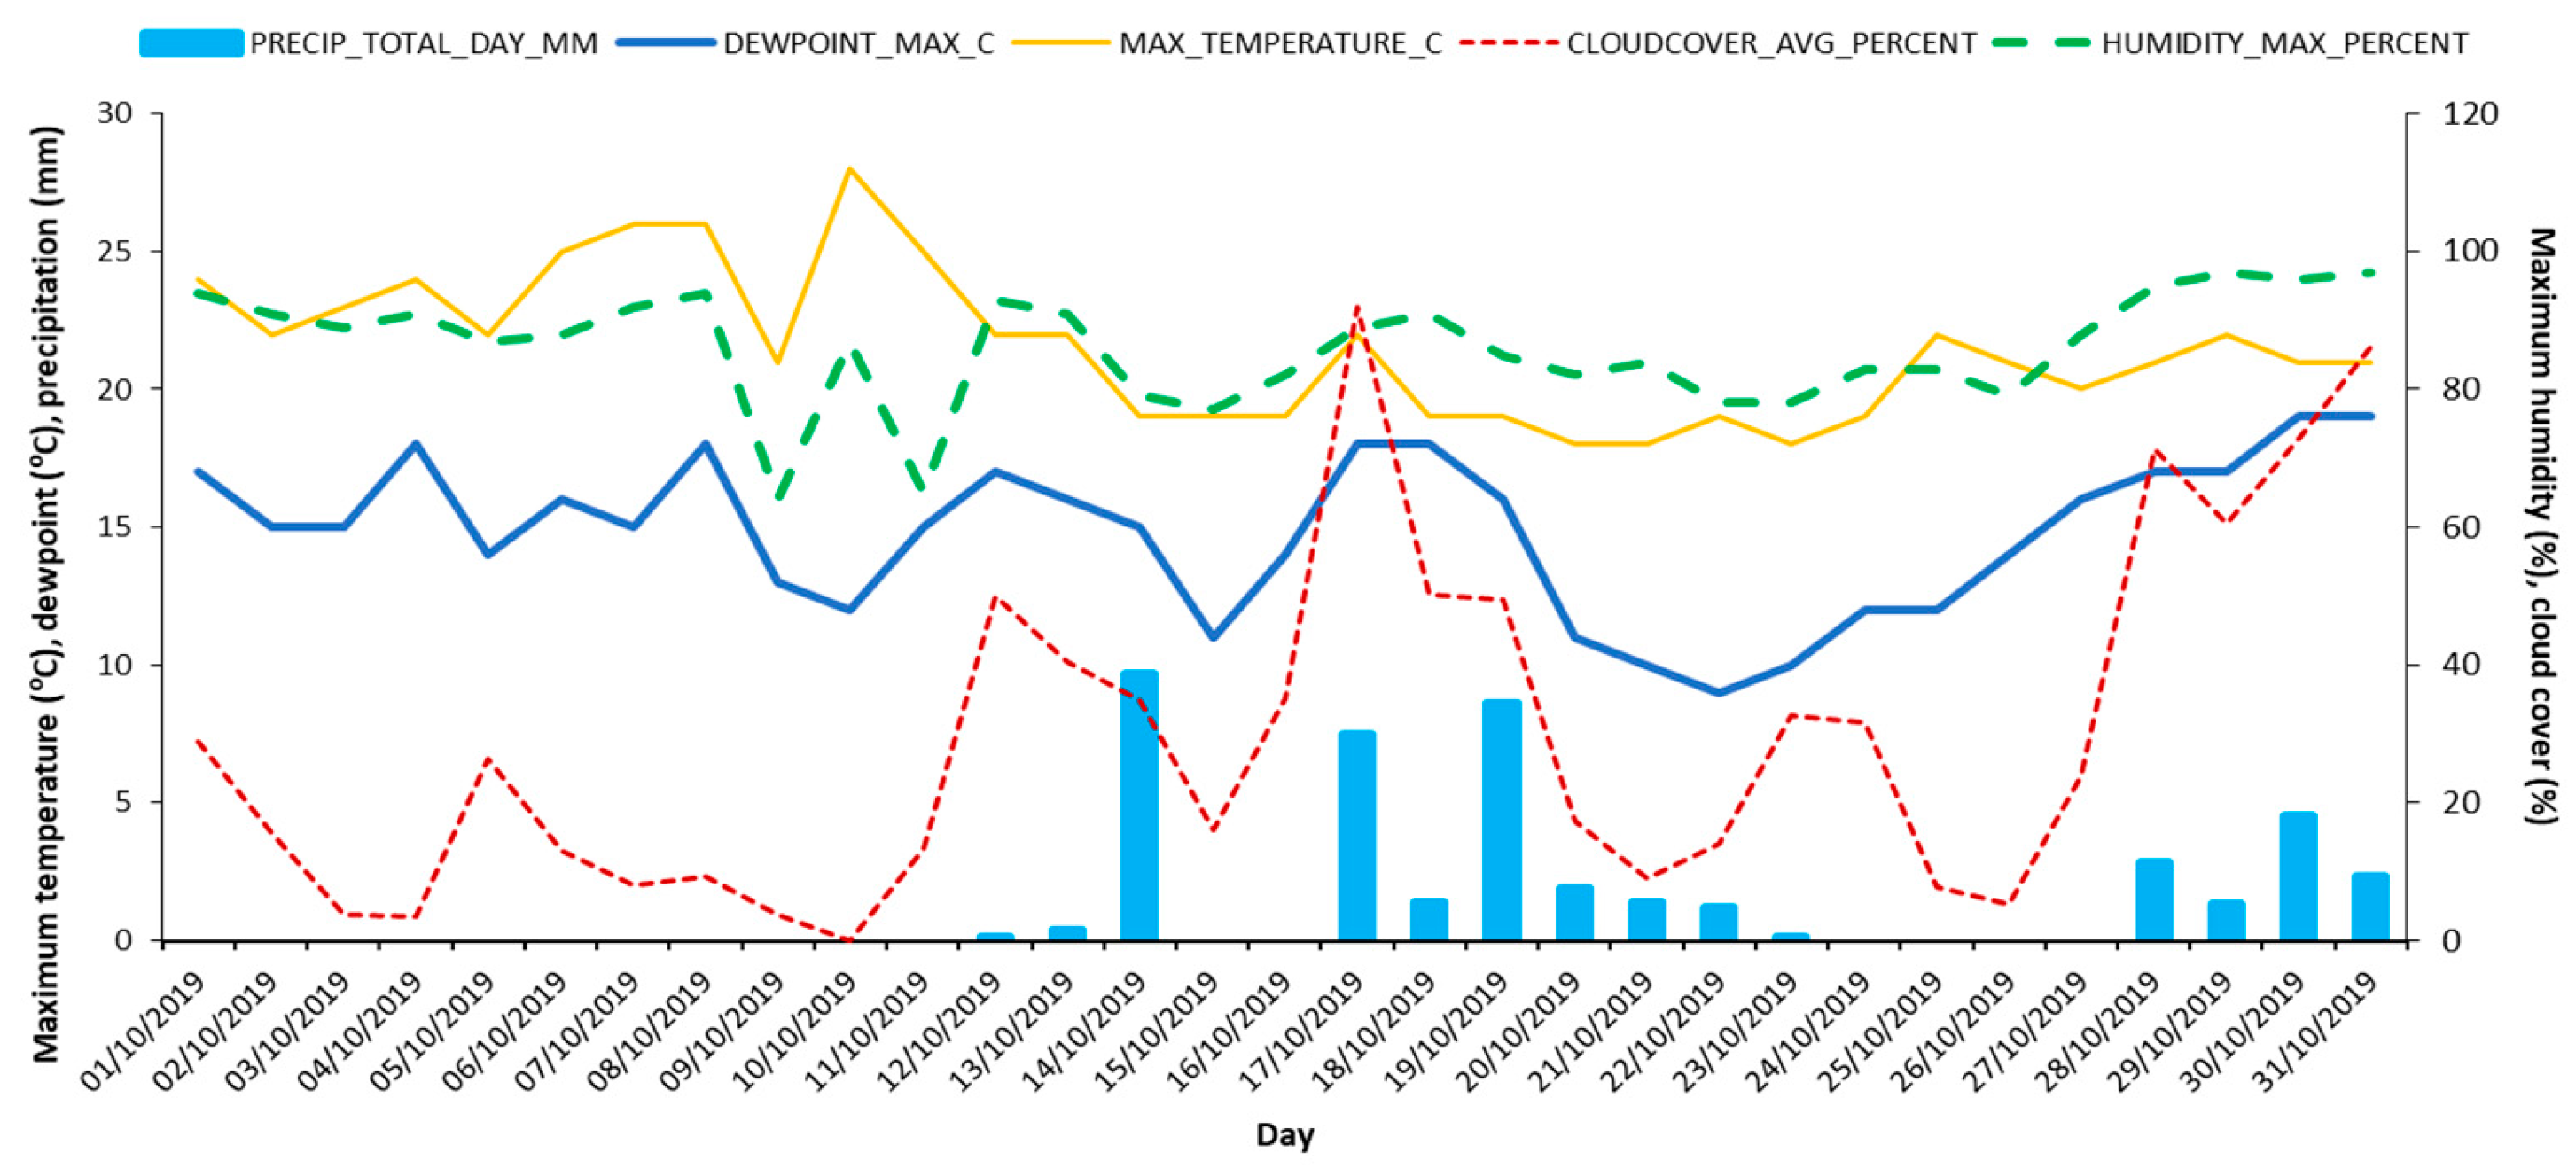
According to the Köppen–Geiger climate classification [26], the study area has a warm temperate climate (Csa), with dry and hot summers and mild winters. For the exact location, average annual precipitation is about 700 mm, ca. 5% of which falls in summer and the remaining 95% distributed in the nine cooler months, a typical Mediterranean climate (https://www.ipma.pt/bin/file.data/climate-normal/cn_91-20_LISBOA_TAPADA.pdf, accessed on 14 October 2025). Indicative environmental conditions during the experimental period are presented in Figure 2 and Table 1.
Figure 2.
Indicative data of daily precipitation (P), maximum dewpoint, maximum air temperature, cloud cover (%) and maximum relative humidity (%) for October 2019 in Lisbon, Portugal (source: weatherspark.com, AWS IPMA Lisboa-Gago Coutinho, at Humberto Delgado Airport, accessed on 14 October 2025).
Table 1.
Selected meteorological variables for the 3rd 10-day period of October 2019, from Gago-Coutinho station, Lisbon, Portugal (Tmin—average minimum daily temperature; Tmax—average maximum daily temperature; Prec—cumulated precipitation; RH—average daily relative humidity; u—average daily wind speed at 10 m height).
2.3. Irrigation Scheduling
Plants were maintained for several months after root division to ensure complete establishment, canopy development, and physiological stabilization, before the onset of the experimental treatments.
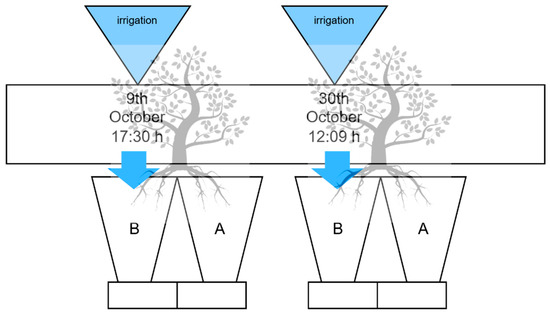
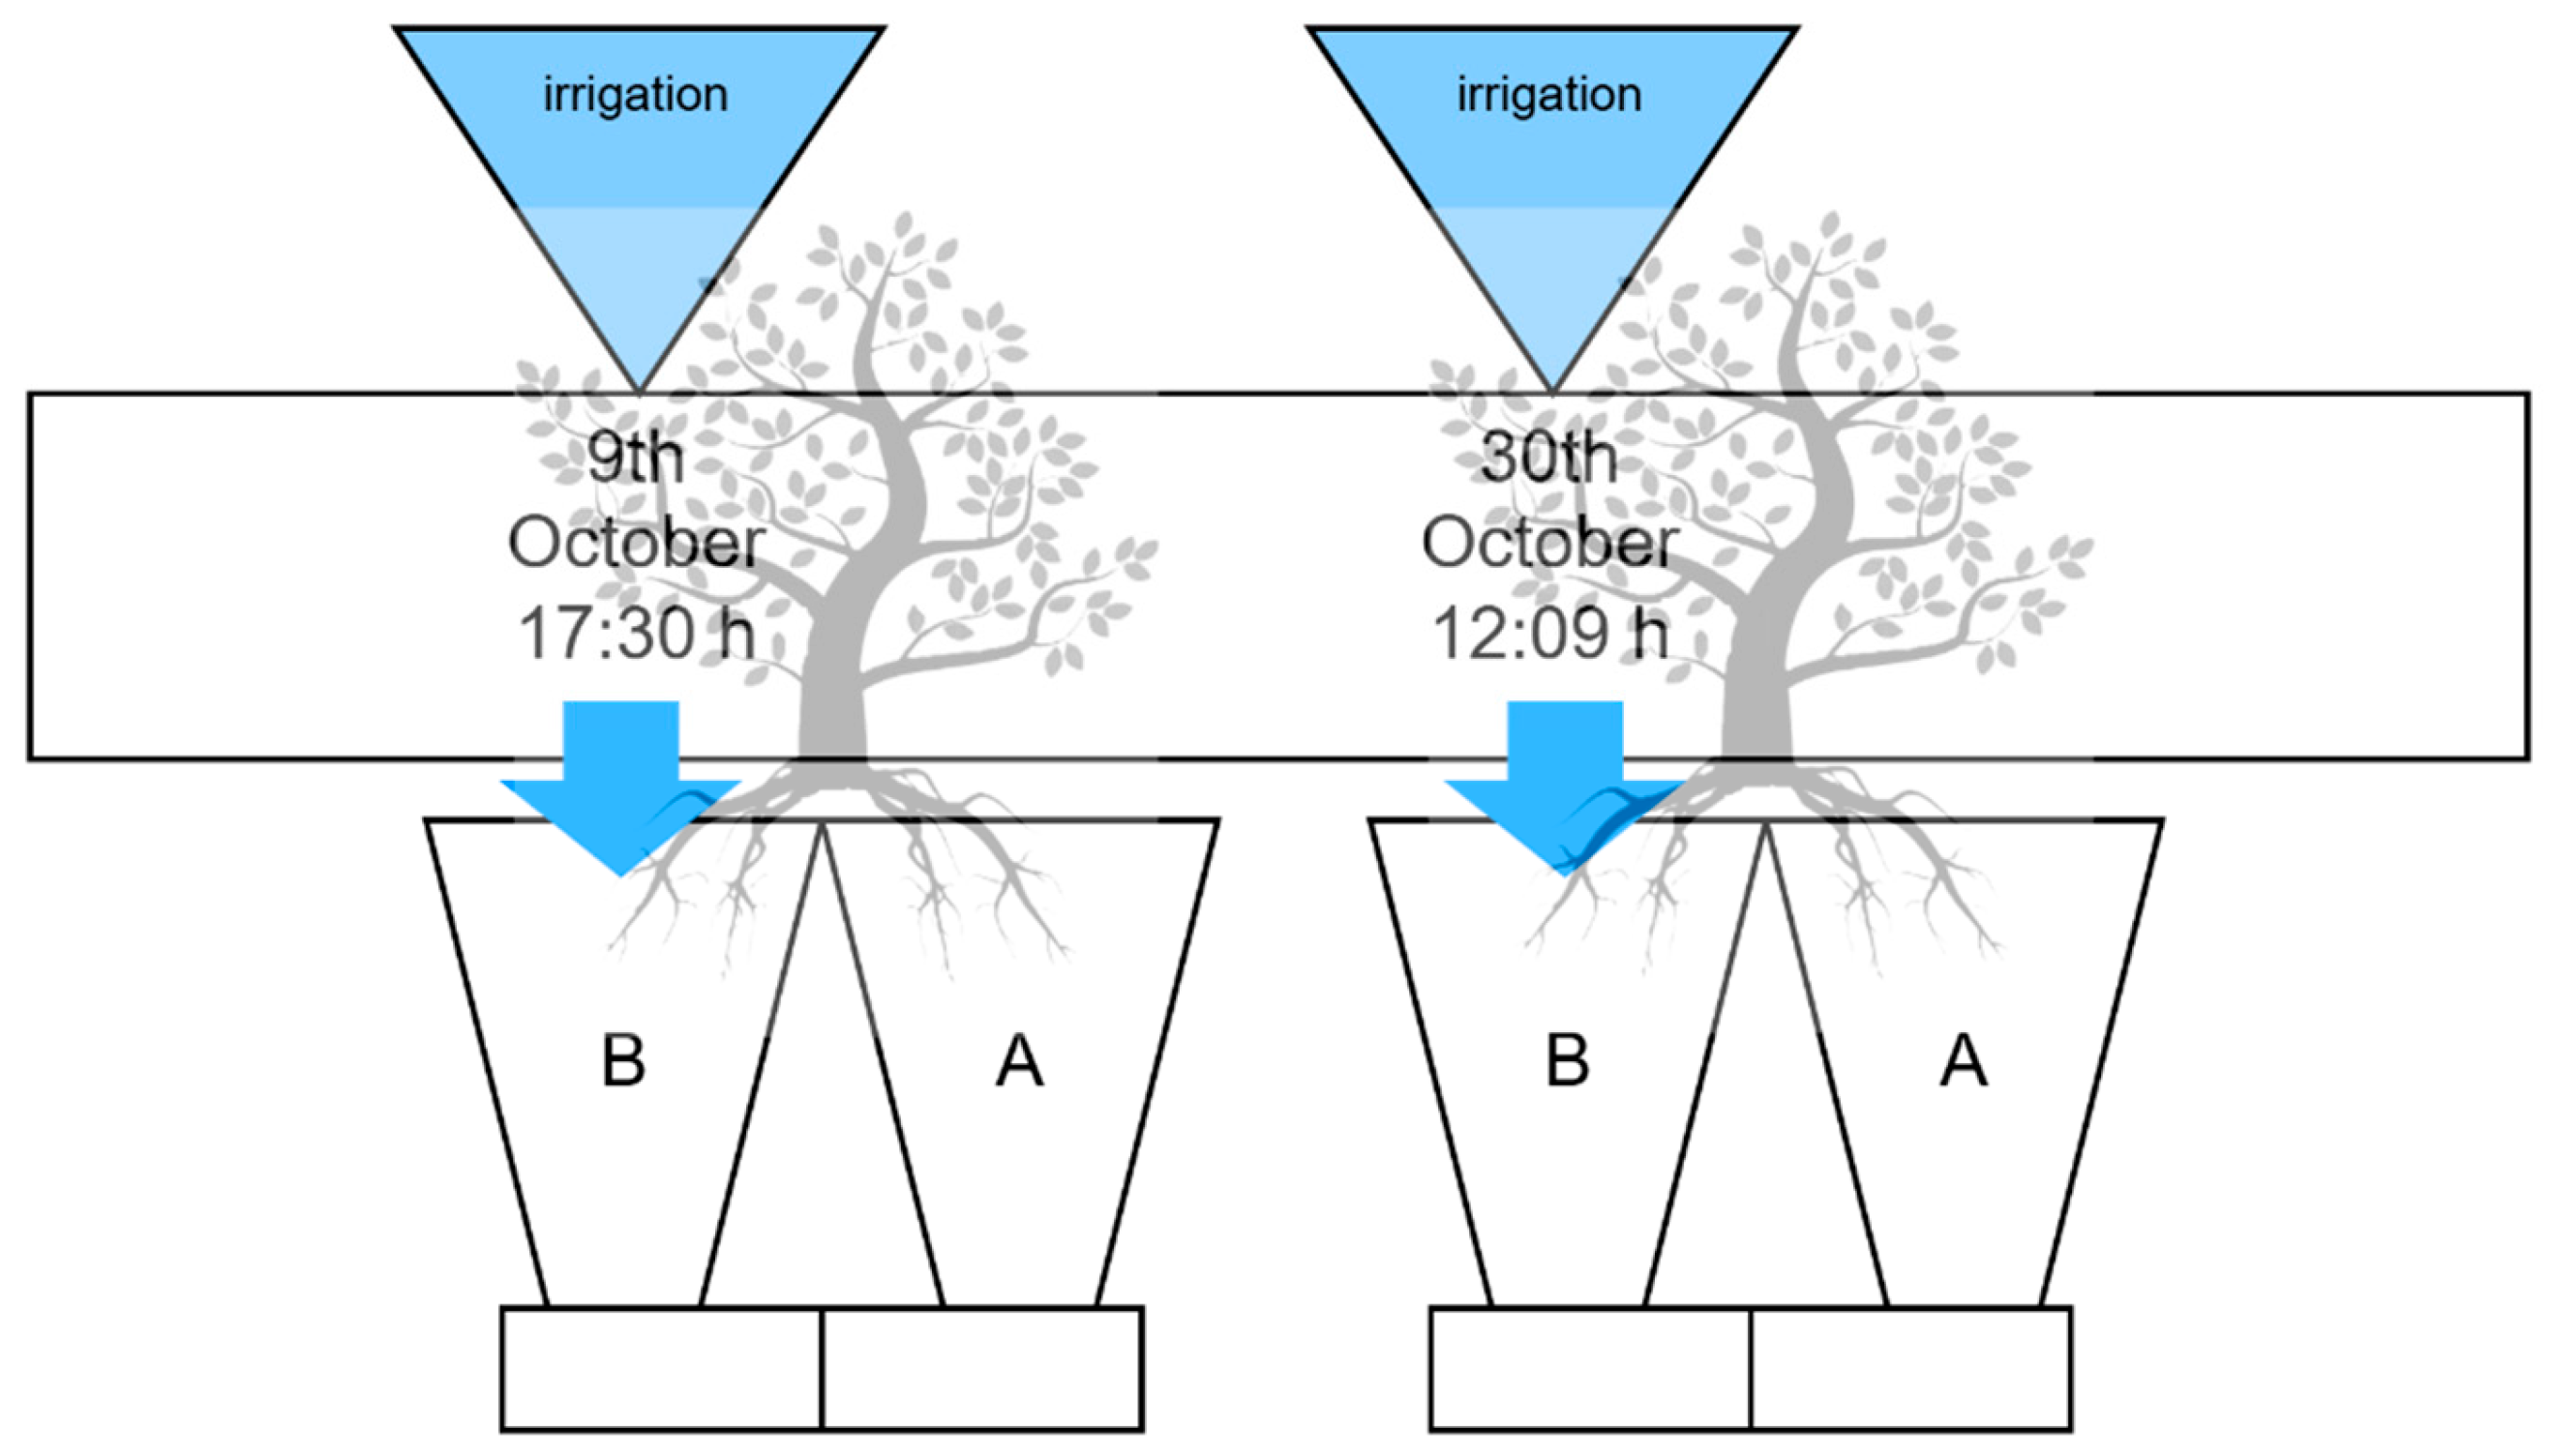
During the stabilization period, irrigation was supplied automatically by drip emitters until 4th October, under progressively increasing water deficit conditions. Throughout the subsequent experimental trial, irrigation was applied manually according to a partial root-zone drying (PRD) protocol, in which water was alternately delivered to only one of the two root compartments while the other was allowed to dry out.
Not all of the five irrigation events of October yielded usable data due to various disturbances at the experimental site. The results presented here correspond to two irrigation events applied exclusively to the B pots, as follows (Figure 3):
Figure 3.
Diagram indicating irrigation events and schematic split-root experimental set with each plant contained in two pots (A non-irrigated and B irrigated).
- -
- On 9 October at 17:30 legal time (500 mL), data analyzed over the 9–10 October period;
- -
- On 30 October at 12:09 (250 mL), data analyzed over the 30–31 October period.
In between there were three other irrigation events of 550 mL in total, per pot. Due to the lockdown periods associated with the COVID-19 pandemic, the experiment could not be continued, as planned, in the following year.
2.4. Precision Weighing Lysimeter Assemblage
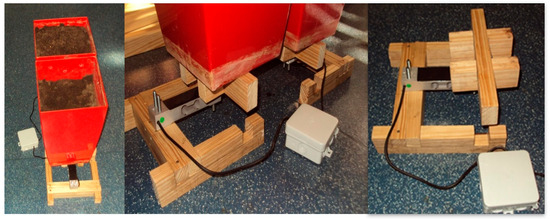
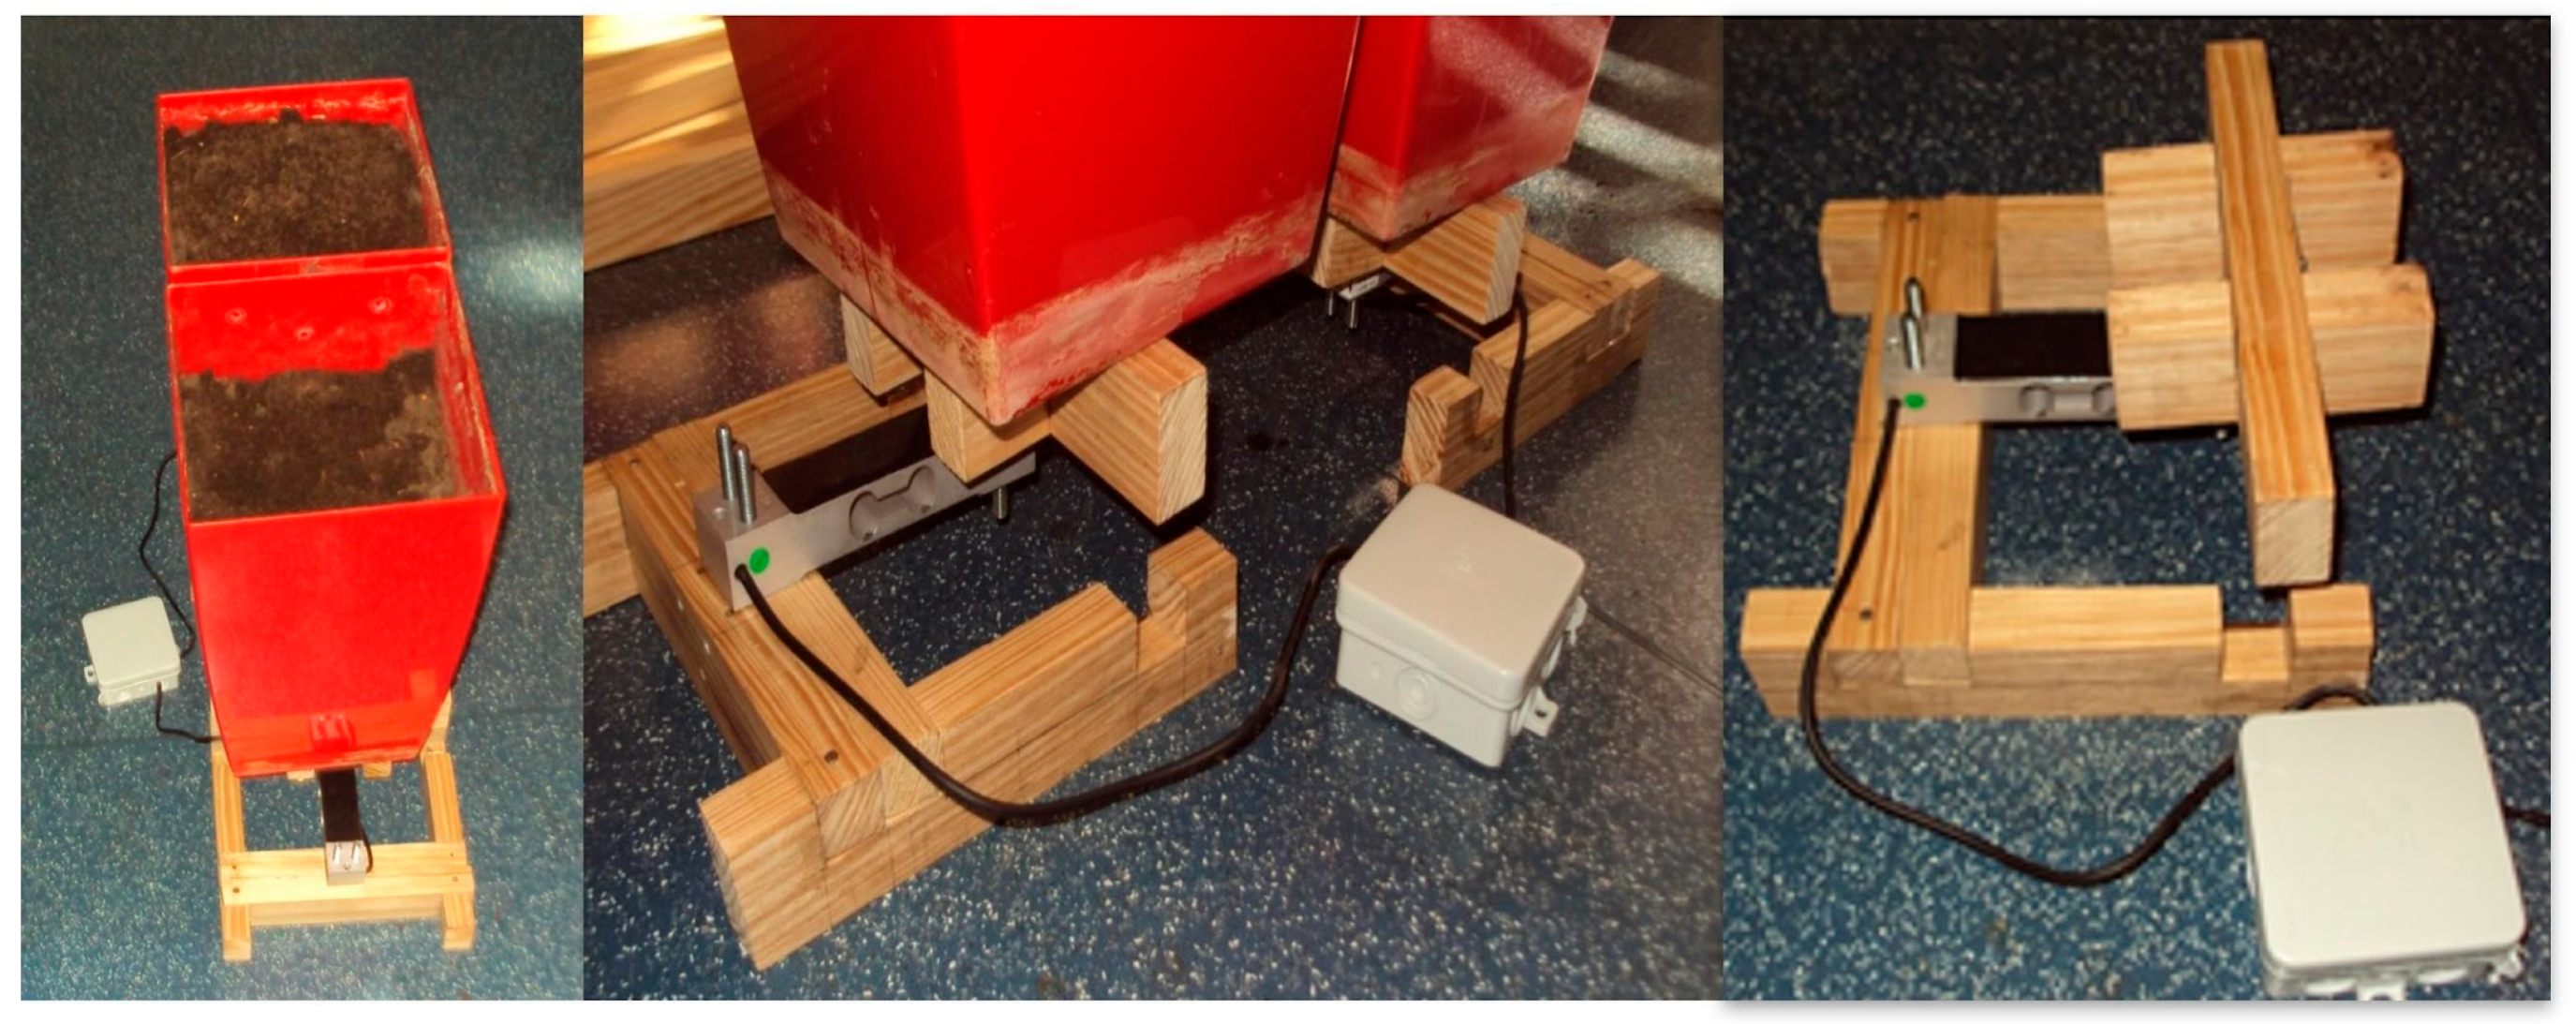
Lysimeters were built using load cells (PA06—Beijing True-Tec Co., Ltd., Beijing, China) with accuracy level equal to ± 0.008% to 0.0116% of full scale, class C6 resolution, with 2.0 mv/v sensitivity and maximum capacity equal to 20 kg, mounted in a wood frame (Figure 4). Each pot within a pair was placed over one unit, constituted by a load cell and a wood frame. The platform–load cell assemblies were specifically designed for this experiment to ensure complete independence in the measurement of the mass of each pot, despite the fact that they were linked two-by-two through the mechanical connection at the base of each plant’s trunk (Figure 2). The data were collected on a CR3000 datalogger (Campbell Scientific, Inc., Logan, UT, USA) and stored every minute.
Figure 4.
Precision weighing lysimeters mounted in a platform with load cells.
3. Results and Discussion
3.1. Time-Series Evolution of Hydraulic Redistribution Processes After First Irrigation
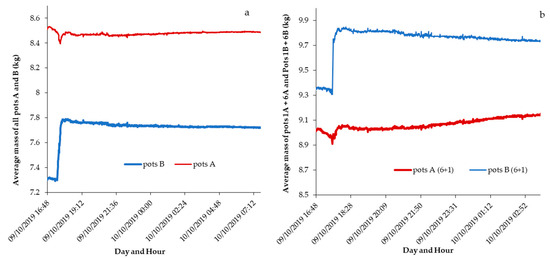
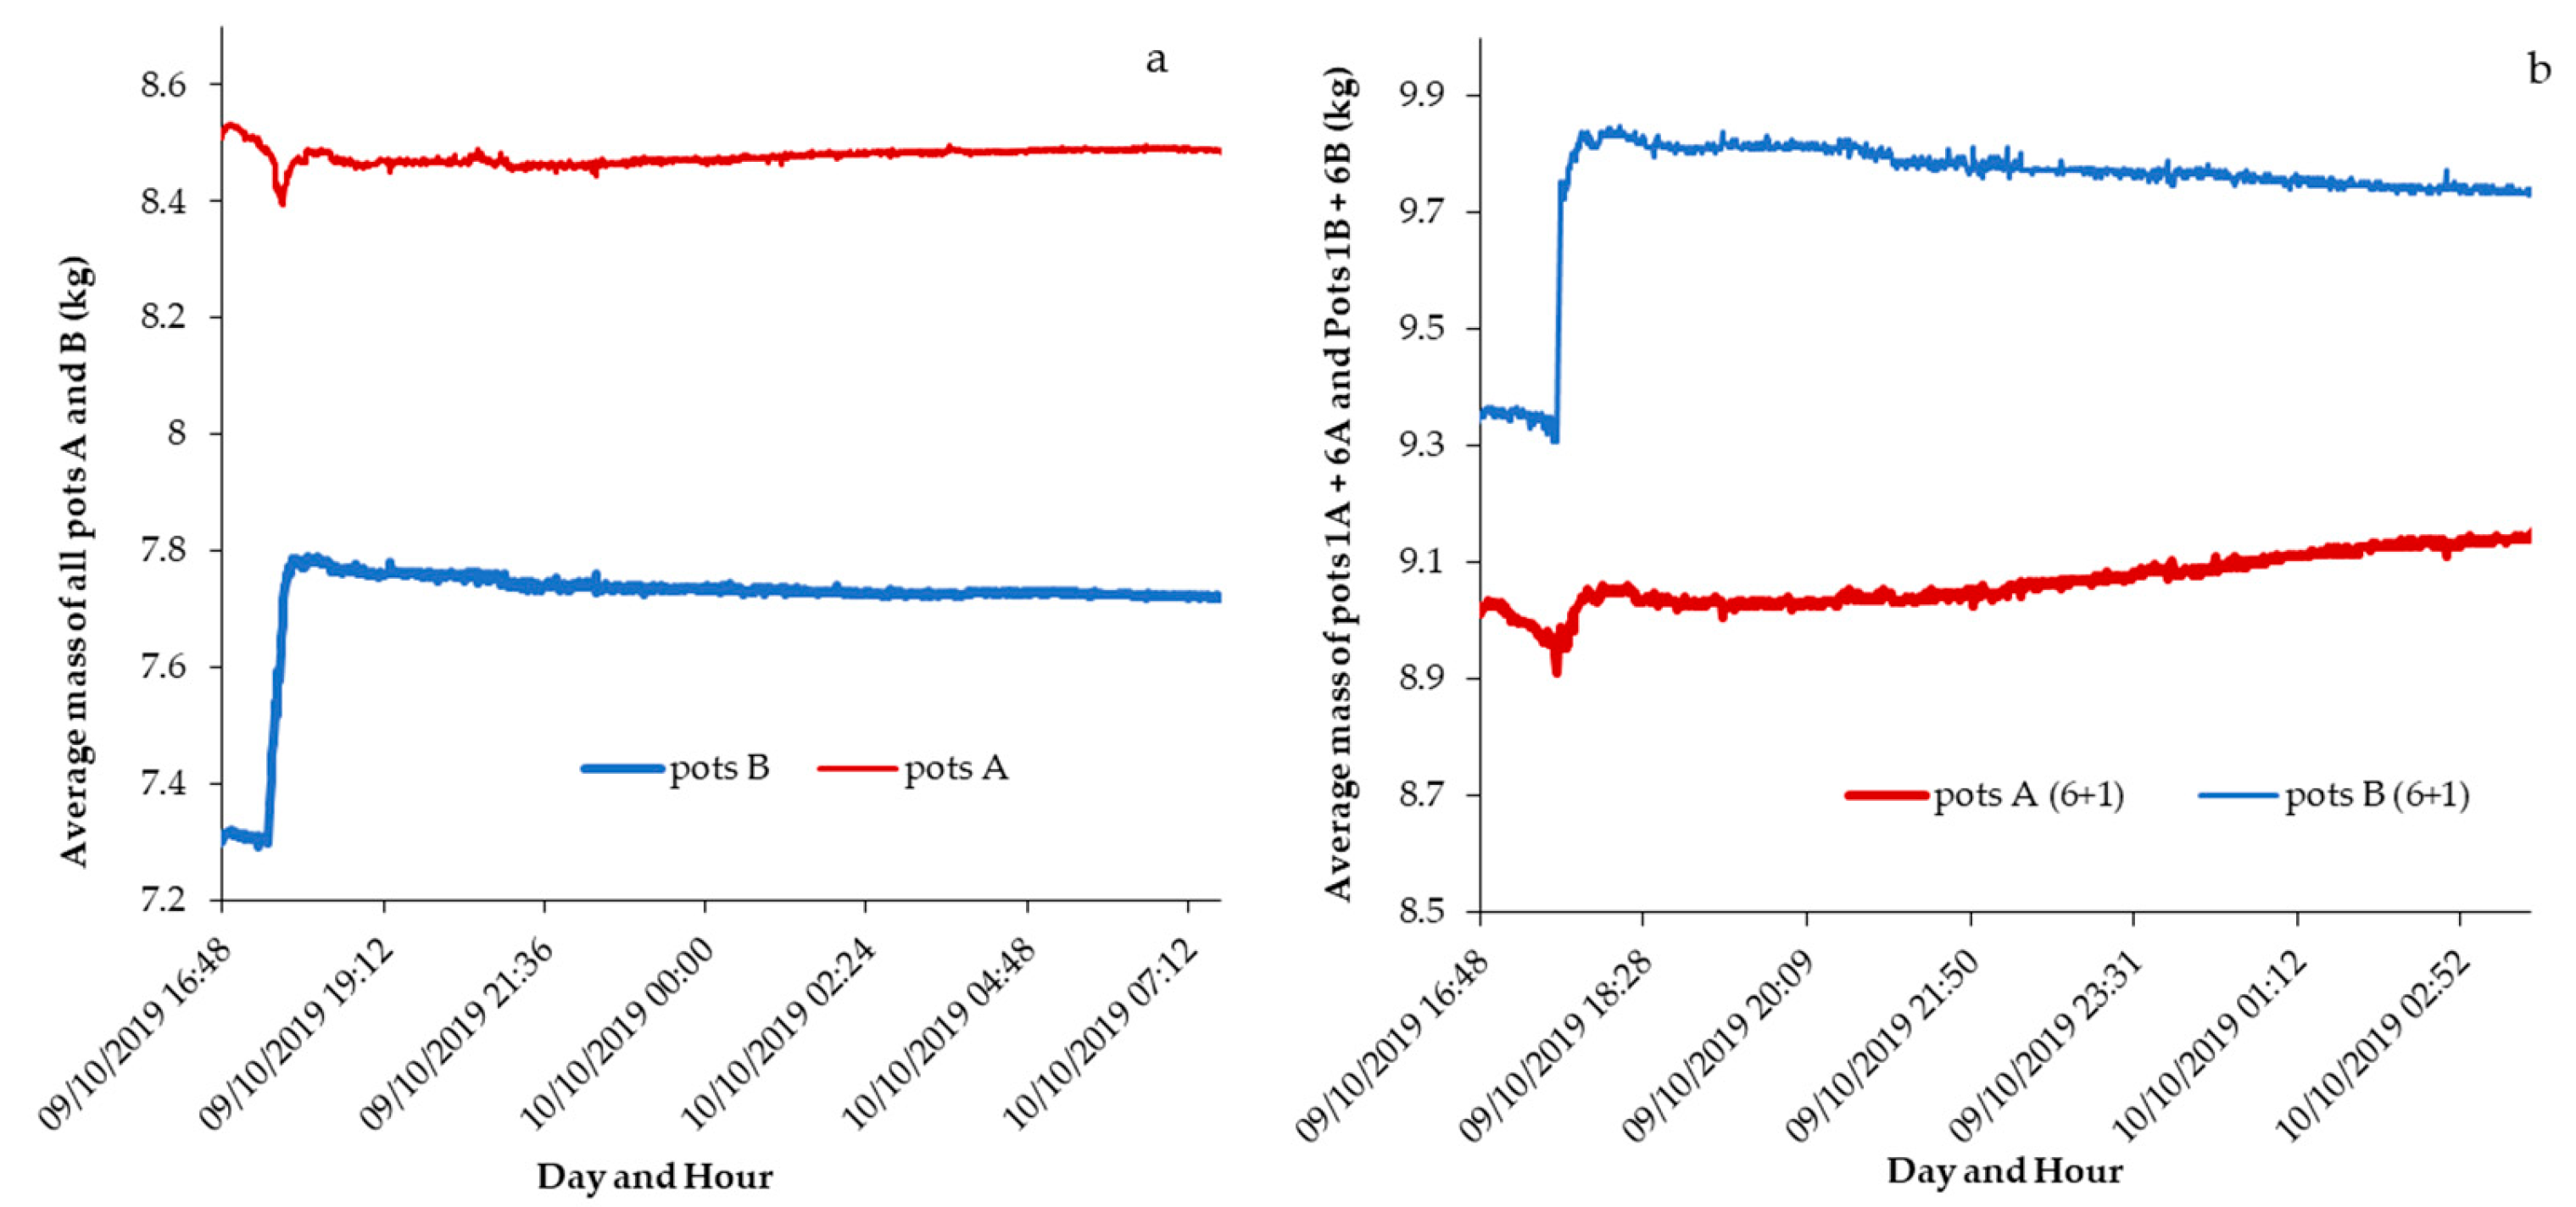
Following the first irrigation of the B pots (17:30, 9 October, application of 500 mL) a sudden change in their mass was recorded, closely matching the applied volume. This observation suggests an accurate functioning of the weighing system. More notably, an increase in the total mass of the A pots was observed over a period of approximately 13 h, accompanied by a decrease in the mass of the B pots (Figure 5a). This strongly suggests that there was a quantifiable movement of water from B to A pots, via roots, which is an important result, confirming water transport from the irrigated to the non-irrigated side of the plants.
Figure 5.
Mass changes for A and B pots, after irrigation in pots B: average for all pots (a); average of pots 1 and 6 (b). Hour is legal summer time (1:45 h later than solar time).
The highest rate of mass transfer occurred during the 13 h period following irrigation (Figure 5a). Afterwards, HR through the roots diminished or ceased. In fact, during the day, the lower water potential would be in the atmosphere and no longer in the soil–root interface in pots A.
In certain pairs of pots, the magnitude of water transfer was markedly greater than in others. For instance, between pairs of pots 1 and 6, the mass of the two A pots increased on average about 0.1 kg for a period of about 10 h (Figure 5b), while the two B pots decreased about 0.1 kg, which corresponds to an overall rate of 10 g per hour. Considering all pots, this value was lower, as indicated below.
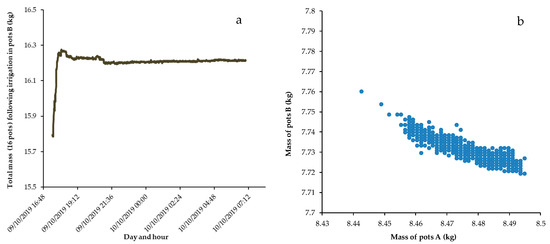
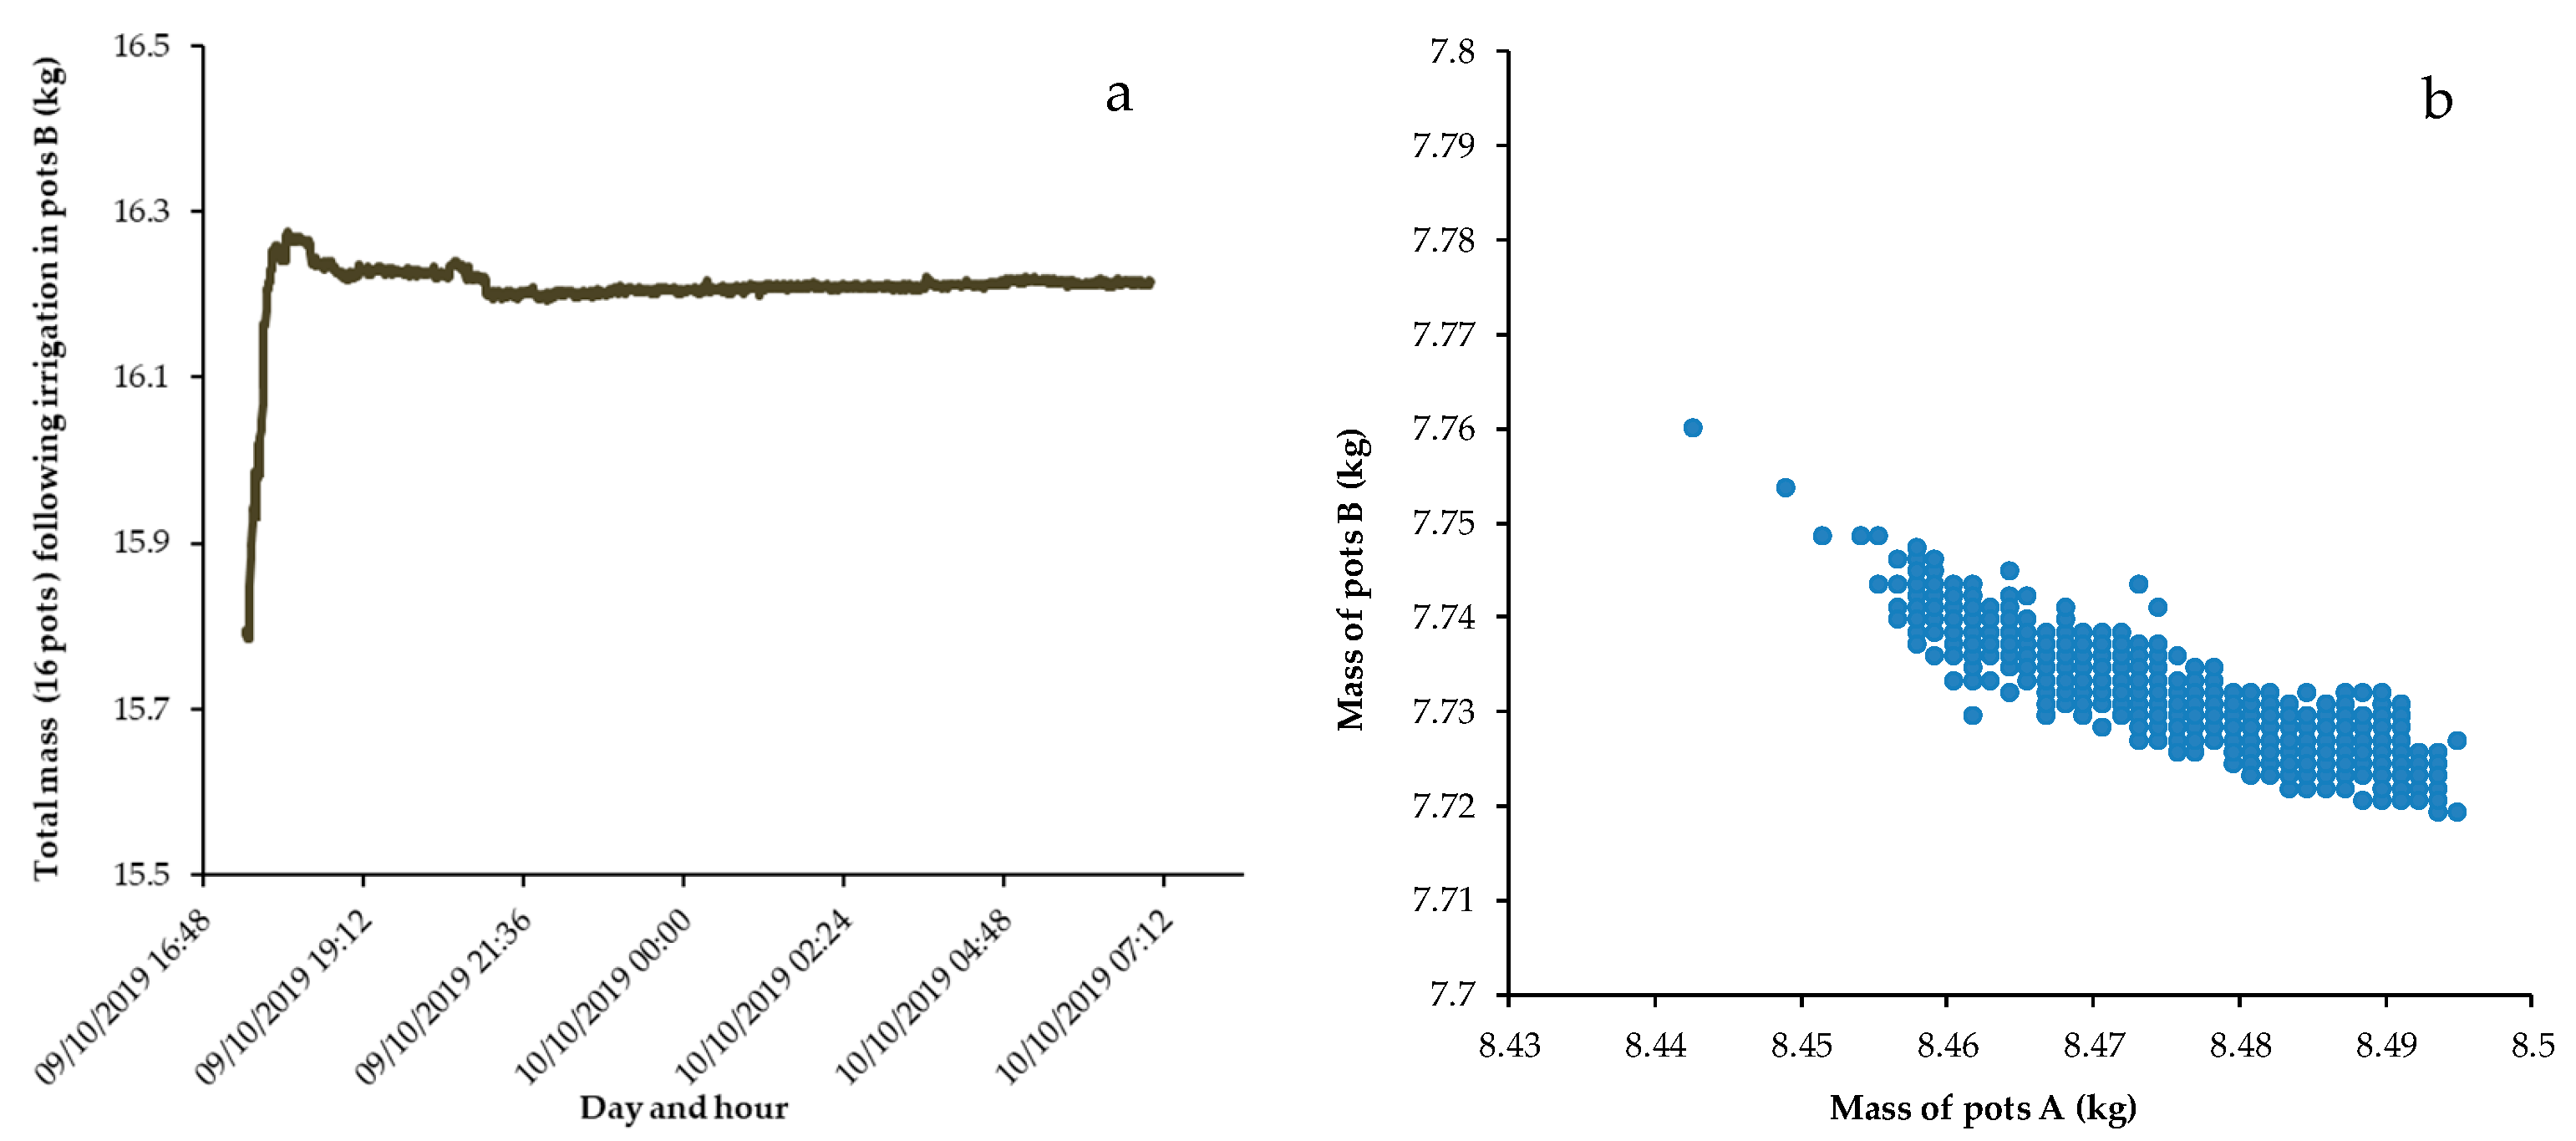
It is anticipated that evapotranspiration (ET) constitutes a component of the total observed mass transfer. Indeed, by summing up the mass of the 16 pots, a loss of weight is visible during the first hours after irrigation (from 17:30 to 21:00 h legal summer time, which was 15:45 to 19:15 solar time) (Figure 6a). This decrease is likely due to ET losses from leaves and soil surface from all pots and on average corresponded to 40 g per pot for such a time period. The analysis for the following nocturnal period is useful, as the ET effect during this period is expected to be small, and does not interfere with mass changes resulting from water redistribution between a pair of pots. Consequently, during the night, as observed in Figure 5a, the total pots’ weight became relatively stable. Although night-time transpiration can occur, in this case we observed it as negligible, likely due to night-time elevated air humidity (even for daily values, average relative humidity was 70% to 90%: location very near to the Atlantic Ocean).
Figure 6.
Mass evolution after irrigation in pots B for (a) the sum of A and B pots (n = 16) and (b) relationship between mass in pots A (gain) vs. pots B (loss), for all pairs of pots (n = 8).
The relationship between losses from pots B and gains of pots A (Figure 5b) reinforces the evidence of HR between the two groups, with a good correspondence between opposite changes in both.
From 21:30 to 7:00 h of 10 October, out of the 500 g of water received, group B lost on average 40 g of water, while group A apparently gained 15 g more (55 g), likely due to night condensation (Figure 6b), which seemed to occur mainly in the dry pots. This is eventually due to higher temperature decrease at the surface (less water, less heat capacitance). Indeed, the total weight (A + B) slightly increased during the night by the same 15 g (Figure 6a).
This group of results suggests the reliability of the experimental design.
3.2. Time-Series Evolution of Hydraulic Redistribution Processes After Second Irrigation
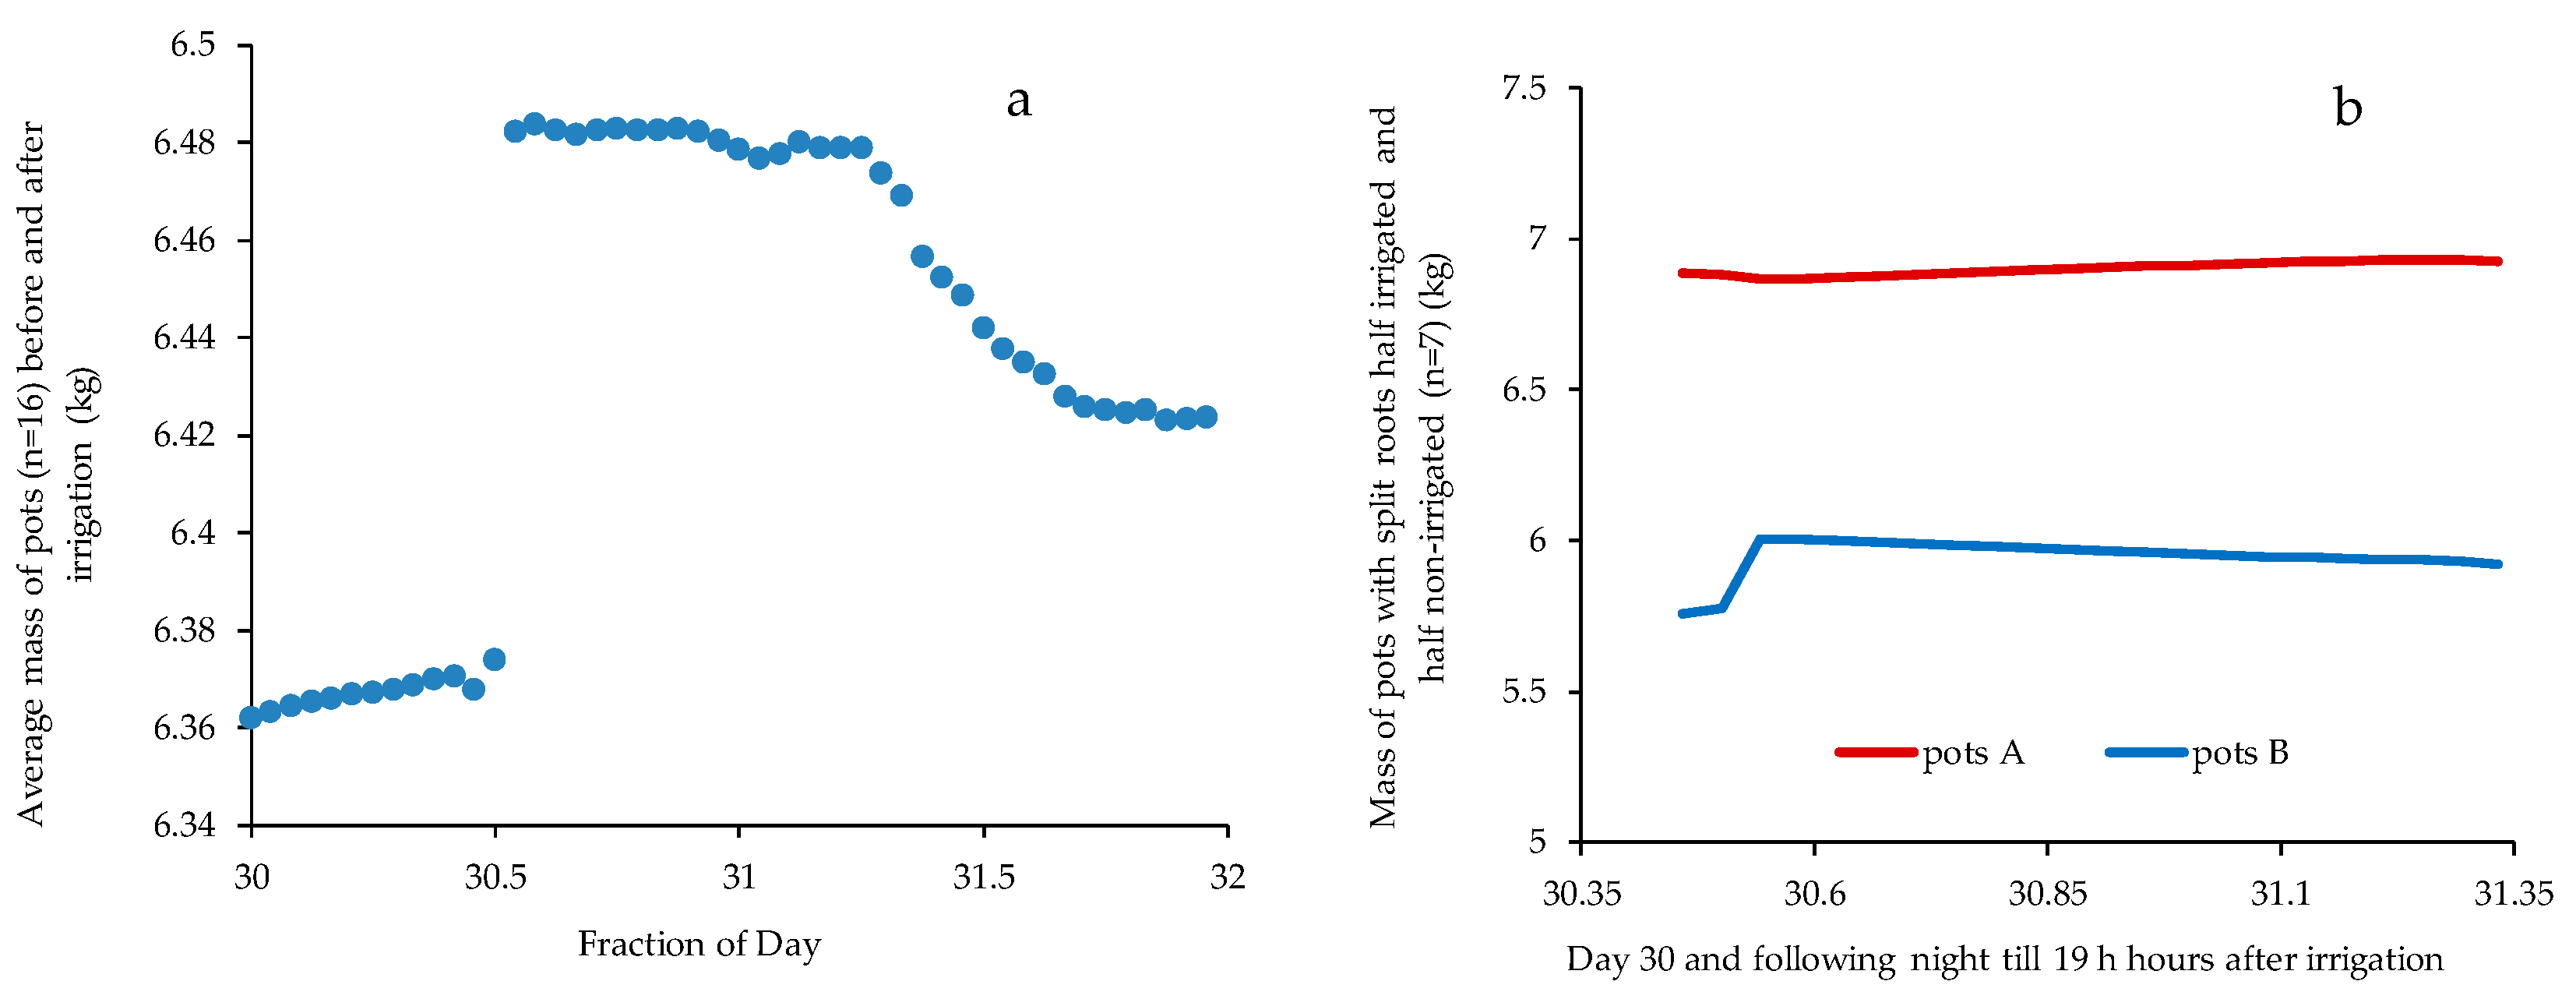
The irrigation of 30 October, at 12:09, on pots B was applied to soil with a much higher level of water stress than the previous one on 9 October, as there was a decrease in the recorded weight throughout the period of the experiment (whole of October). The average pot mass decreased from 7.9 kg (Figure 5b) before the irrigation of 9 October to 6.4 kg before the irrigation of 30 October (Figure 7a), in spite of three other intermediate irrigations in between, as mentioned above. This indicates that, as intended, the applied deficit irrigation did not fully compensate for the water mass lost through ET. This aspect is crucial to understand the nuance in results, as compared to the previous period.
Figure 7.
Average mass (hourly values) before and after irrigation of (a) all 16 pots, from 30 October up to the end of 31 October (the difference in mass after irrigation appears divided by two, 125 g, as water was applied only in 8 pots) and (b) for separated groups A and B (n = 7), up to early morning of 31 October.
Surprisingly, the line for the afternoon of 30 October (total mass of all pots) does not show the clear slope one could expect if ET occurred (Figure 7a). This indicates reduced water use during that first afternoon, opposite to the sharp decrease in mass observed during day 31. This pattern was consistent across all pairs of pots.
As before, the change in mass in pots A was compared with the equivalent mass in pots B (Figure 7b) where only seven pairs of pots were considered (one was not functioning well). It can be seen that when irrigation was applied to pots B, there was an increase in the mass of pots A over a period of 17 h (up to the early morning of 31 October) accompanied by a decrease in weight of pots B. Therefore, water transport from the irrigated side to the non-irrigated one of the plants was again observed.
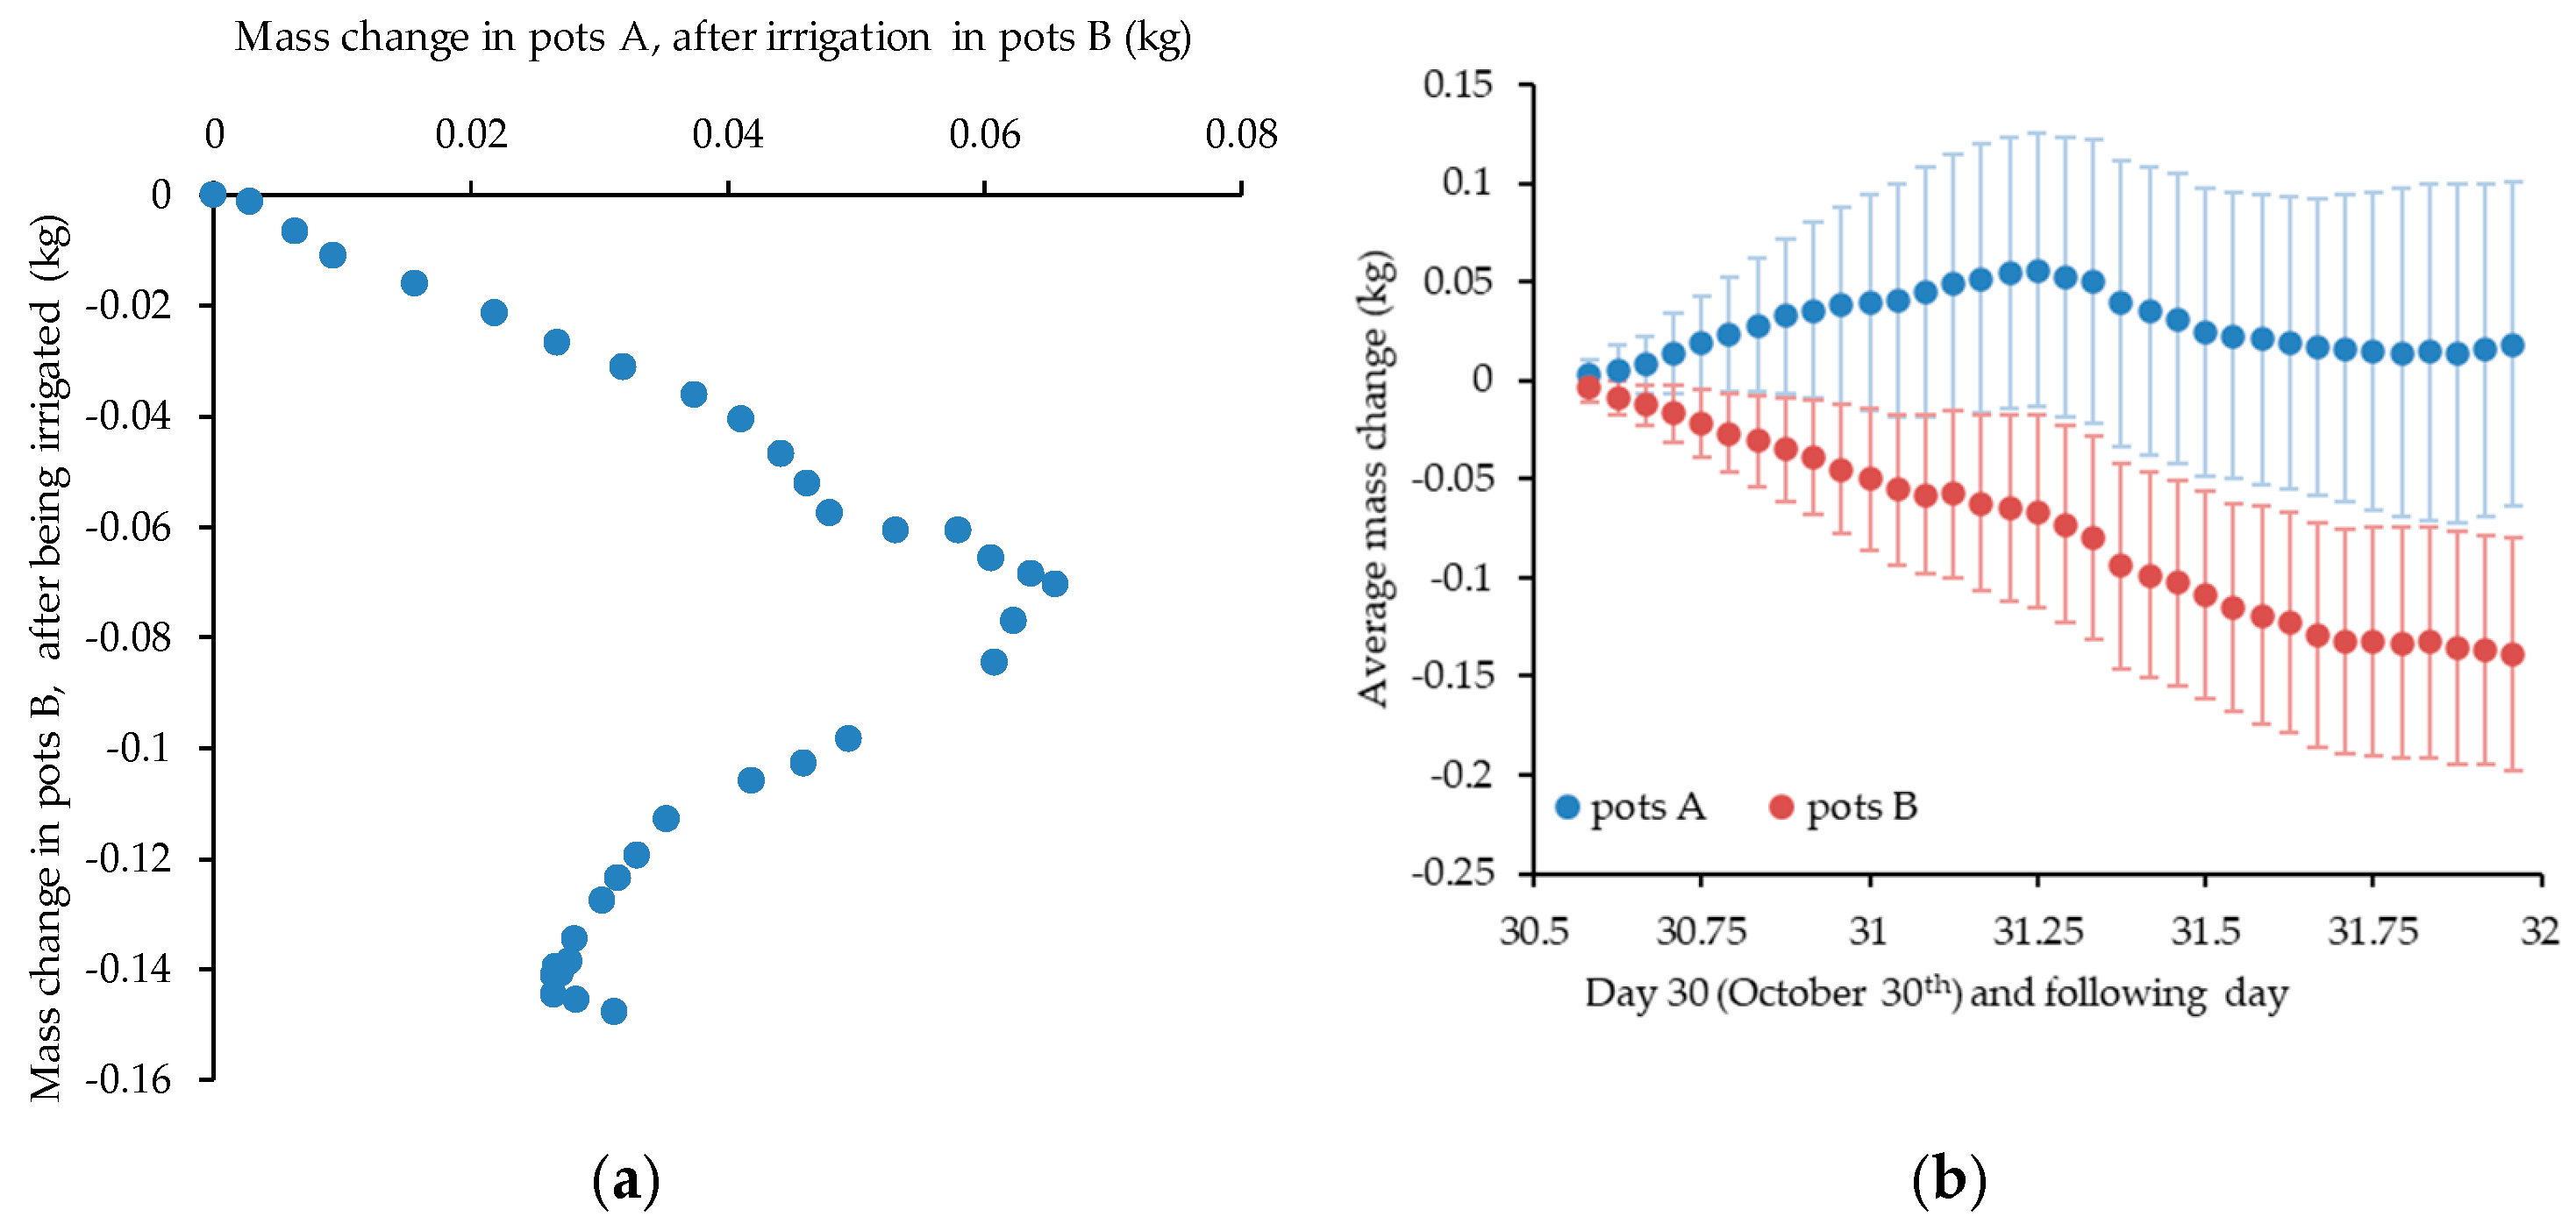
During this period, and as before, there is a negative correlation between the two data series. The relationship between average mass changes in A and B groups is presented in Figure 8a, up to 6:00 in the morning, and mean and standard deviations of mass change are presented in Figure 8b. When the daylight hours of 31 October began, both groups of pots lost weight simultaneously, with a positive slope in the relationship between the masses, suggesting that during daylight on 31 October, the redistribution of water through the roots was highly reduced and both groups lost mass in parallel, due to ET (also clear from total mass loss in Figure 7a). For the first night hours of 31 October, the slope inverted again.
Figure 8.
(a) Relationship between average mass changes (n = 7) in A and B groups after irrigation, in three steps: (1) during the first 17 h after irrigation of B pots (i.e., first afternoon and following night), (2) until water uptake occurs mostly to the shoot during the day and early night, and finally (3) new inversion of slope as the second night progresses (after 9:00 pm, i.e., 19:15 solar time, 31 October); (b) mean and standard deviations of mass change of pots A and B (n = 8).
Figure 8 clearly indicates the progressive mass gain in pots A, coming from water redistribution from pots B, which attained 66 g for the rest of 30 October and the following night, corresponding to a similar mass loss of pots B (70 g). This suggests ET would have been residual (70 − 66 = 4 g) for that day.
Pots B constantly lost water mainly up to the start of the second night, when water redistribution was highly reduced. During the daylight hours of 31 October (second day), pots A lost on average 39 g (0.066–0.026 kg) and pots B lost even more, 74 g (0.145–0.070 kg).
The larger water losses in pots B occur since these losses provide water both for redistribution within pots A and for ET (ET with a higher rate than from pots A, since plants are not as stressed as the ones in pots A). This is dissimilar from pots A, which are simultaneously gaining water from HR, sourced from pots B. The total loss for pots B since irrigation (30 October) up to 11 pm (31 October) was 148 g, out of the 250 g received in last irrigation. The net gain for pots A was 31 g.
Therefore, the total ET during 31 October daylight hours (pots A and B) would be 113 g, as 39 g was the sum of HR gain for pots A minus its ET, and 74 g was the HR loss from pots B, minus its ET, in contrast with the very low value of the proceeding afternoon. At a first glance, this observation underscores the necessity of conducting a comparative analysis of the meteorological conditions prevailing on the two relevant days.
In fact, the available data do not permit a reliable estimation of ET within the greenhouse environment. One can consider that the external conditions were different in relation to those prevailing on the previous days, with higher maximum humidity, maximum dew point, greater cloud cover (Figure 2) and the occurrence of precipitation, thus being a period of high humidity and low radiation in general. Temperature was similar between the two days. The only important difference was in precipitation, which was higher on 30 October. It is clear that the conditions, both the ones described and the reports from the IPMA services, suggest a period of low ET. However, it is not clear that these differences justify the distinct ET rates of both days.
Another more interesting hypothesis could be the reduced transpiration activity of irrigated pots, very soon after irrigation, when the lower water potential in the system is found in the extremely dry soil, towards where water moves, rather than in the very humid atmosphere. Therefore, no important transpiration would occur, with soil evaporation being also negligible or negative (condensation). Conversely, during the second day, the contrast of water status in both groups of pots would be less dramatic and more water would be moving to the atmosphere. As mentioned by Thomas et al. [28] in a study with maize, in case of dry nights, the night-time transpiration and xylem refilling override HR on a diurnal basis. The present situation is opposite to this, as air was almost saturated during the night.
3.3. Observed ET Rates with Lysimeters Versus Estimates
A last step is to infer, from the limited knowledge and data available, the expected ET loss during such days, in such specific conditions.
The ET rates can be obtained from the changes in time of the total mass of all pots. The values observed were compared to approximative estimates of ET rates obtained using the leaf area of the young trees. To our knowledge, studies with olive trees in greenhouses are rare and we have used data from studies in open fields.
Measurements over several years in an irrigated olive orchard [14] suggest ET well below 1 mm/day, and ET in relation to reference ET between 0.1 and 0.2, for this time of year (October to November). The authors indicate a leaf area index of about 1 (m2 of leaves per m2 of total soil or social area of each plant), meaning that a limit value of 1 mm/day corresponds to 1 L/m2 of leaves. As the plants are not rooted in soil, but potted, the relationships were applied via leaf area of the leaves of each tree, evaluated as described above.
In addition, consulting reference ET data for Lisbon (ETo), it is possible to observe a value of 20.5 mm for the last 10-day period of October 2019 [27]. Using the average ETo for these 10 days and 0.1 to 0.2 as ET/ETo, ET of olive leaves in open air would be below 0.1 to 0.2 L/m2 (of leaves).
Consequently, a possibly reasonable estimate for ET, if these trees were in open air, could be on average 30 to 60 g per day and per average tree in pots (for 0.3 m2 of leaves per tree). This rough estimation provides an indicative range, which is similar to the measures for potted trees above for 31 October, of 113 g.
The value of 40 g for 9 October, when temperature was higher, cloud cover lower and precipitation absent, is also in the same order of magnitude, since it refers only to the period after 17:30. Considering the application of 1050 g of water between 9 October and the morning of October 30, and the mass loss of 3000 g in this interval, the average ET is about 193 g per day and per pot, likely decreasing from the beginning of this period towards the end, due to increasing water stress and decreasing water demand of the atmosphere. If estimates are reliable, it could be inferred that ET was higher inside the greenhouse, in spite of the lack of significant convection.
4. Conclusions
In the present study, the hydraulic redistribution between separated roots of the same olive plant (in A and B pots) was measured with weighted lysimeters: a quantifiable movement of water via roots, from irrigated pots (B) to pots where water status was very low (A), was observed. These results confirm the departing hypotheses: (i) HR occurs in split-root olive plants between the irrigated and non-irrigated halves of the root system; (ii) the high-precision weighing system is able to detect and measure HR.
The intensity of the transfer by HR decreases after its start, following irrigation, being especially apparent during the following night. HR rate attained 10 g per hour for some pots and was 40 g and 66 g, on average, for the night after 9 October (n = 8) and for the night of 30 October (n = 7), respectively.
During a sunny day (9 October), the lower water potential is likely to be found in the atmosphere, and the root to shoot transfer process is dominant. Conversely, during a cloudy and rainy day immediately after irrigation (30 October), HR still dominates in diurnal hours, with residual root–shoot transfer. After the first day of intensive HR, the root to shoot process dominates again with rates of ET of 113 g on average (31 October), taken from the time series of the total mass (all pots), which corresponds to 360 g/m2 of leaves.
The relationship between the mass changes of irrigated pots and mass changes of dry pots is in an inverse proportion at night or on cloudy humid days, when HR dominates (Figure 5b), and in a direct proportion in the day, when ET dominates (Figure 7).
The device used to measure each of the 16 pots showed to be effective in providing the weight of each half root + soil pot independently of the other half root + soil, for the same plant, in spite of the mechanical link between them. Furthermore, the system allowed us to quantify the amount of water that was transferred from the irrigated to the non-irrigated pots, proving the relevance of the HR fluxes. However, these data must be considered carefully, since the experimental work was done under controlled conditions and might differ from field results.
Author Contributions
Conceptualization, M.I.F., J.R. and F.S.; methodology, M.I.F., J.R. and F.S.; software, M.I.F., J.R., F.S. and T.A.P.; validation, M.I.F., J.R., F.S. and T.A.P.; formal analysis, M.I.F., J.R., F.S. and T.A.P.; investigation, M.I.F., F.S. and J.R.; resources, M.I.F., J.R. and F.S.; data curation, M.I.F.; writing—original draft preparation, M.I.F., J.R. and T.A.P.; writing—review and editing, M.I.F., J.R., F.S. and T.A.P.; visualization, M.I.F., J.R., F.S. and T.A.P.; supervision, M.I.F.; project administration, M.I.F.; funding acquisition, M.I.F. All authors have read and agreed to the published version of the manuscript.
Funding
This research was funded by project WASA—WAter Saving in Agriculture: technological developments for the sustainable management of limited water resources in the Mediterranean area (ERANETMED/0006/WATER-13-109/2014, CE).
Data Availability Statement
The data presented in this study are available in the article, except for the unpublished data referring to horizontal redistribution in the field.
Acknowledgments
The authors acknowledge FCT (Fundação para a Ciência e a Tecnologia), I.P., under the project UIDB/04129/2025 of the LEAF Research Unit—Linking Landscape, Environment, Agriculture and Food—and Sónia Lourenço for helping in the preparation of the pots and irrigation scheduling.
Conflicts of Interest
The authors declare no conflicts of interest. The funders had no role in the design of this study; in the collection, analyses, or interpretation of data; in the writing of the manuscript; or in the decision to publish the results.
References
- Burgess, S.S.O.; Adams, M.A.; Turner, N.C.; Ong, C.K. The Redistribution of Soil Water by Tree Root Systems. Oecologia 1998, 115, 306–311. [Google Scholar] [CrossRef] [Scilit]
- Caldwell, M.M.; Dawson, T.E.; Richards, J.H. Hydraulic Lift: Consequences of Water Efflux from the Roots of Plants. Oecologia 1998, 113, 151–161. [Google Scholar] [CrossRef] [Scilit]
- Burgess, S.S.O. Can Hydraulic Redistribution Put Bread on Our Table? Plant Soil 2011, 341, 25–29. [Google Scholar] [CrossRef] [Scilit]
- Sekiya, N.; Araki, H.; Yano, K. Applying Hydraulic Lift in an Agroecosystem: Forage Plants with Shoots Removed Supply Water to Neighboring Vegetable Crops. Plant Soil 2011, 341, 39–50. [Google Scholar] [CrossRef] [Scilit]
- Hirota, I.; Sakuratani, T.; Sato, T.; Higuchi, H.; Nawata, E. A Split-Root Apparatus for Examining the Effects of Hydraulic Lift by Trees on the Water Status of Neighbouring Crops. Agrofor. Syst. 2004, 60, 181–187. [Google Scholar] [CrossRef] [Scilit]
- Scholz, F.G.; Bucci, S.J.; Meinzer, F.C.; Goldstein, G. Maintenance of Root Function in Tropical Woody Species During Droughts: Hydraulic Redistribution, Refilling of Embolized Vessels, and Facilitation Between Plants. Trop. Tree Physiol. 2016, 227–241. [Google Scholar] [CrossRef] [Scilit]
- Alagele, S.M.; Jose, S.; Anderson, S.H.; Udawatta, R.P. Hydraulic Lift: Processes, Methods, and Practical Implications for Society. Agrofor. Syst. 2021, 95, 641–657. [Google Scholar] [CrossRef] [Scilit]
- Zegada-Lizarazu, W.; Iijima, M. Hydrogen Stable Isotope Analysis of Water Acquisition Ability of Deep Roots and Hydraulic Lift in Sixteen Food Crop Species. Plant Prod. Sci. 2004, 7, 427–434. [Google Scholar] [CrossRef] [Scilit]
- Quijano, J.C.; Kumar, P. Numerical Simulations of Hydraulic Redistribution across Climates: The Role of the Root Hydraulic Conductivities. Water Resour. Res. 2015, 51, 8529–8550. [Google Scholar] [CrossRef] [Scilit]
- Yang, G.; Huang, L.; Shi, Y. Magnitude and Determinants of Plant Root Hydraulic Redistribution: A Global Synthesis Analysis. Front. Plant Sci. 2022, 13, 918585. [Google Scholar] [CrossRef] [Scilit]
- Nadezhdina, N.; Ferreira, M.I.; Silva, R.; Pacheco, C.A. Seasonal Variation of Water Uptake of a Quercus Suber Tree in Central Portugal. Plant Soil 2008, 305, 105–119. [Google Scholar] [CrossRef] [Scilit]
- Ferreira, M.I.; Green, S.; Conceição, N.; Fernández, J.E. Assessing Hydraulic Redistribution with the Compensated Average Gradient Heat-Pulse Method on Rain-Fed Olive Trees. Plant Soil 2018, 425, 21–41. [Google Scholar] [CrossRef] [Scilit]
- Nadezhdina, N.; Ferreira, M.I.; Conceição, N.; Pacheco, C.A.; Häusler, M.; David, T.S. Water Uptake and Hydraulic Redistribution under a Seasonal Climate: Long-Term Study in a Rainfed Olive Orchard. Ecohydrology 2015, 8, 387–397. [Google Scholar] [CrossRef] [Scilit]
- Conceição, N.; Tezza, L.; Häusler, M.; Lourenço, S.; Pacheco, C.A.; Ferreira, M.I. Three Years of Monitoring Evapotranspiration Components and Crop and Stress Coefficients in a Deficit Irrigated Intensive Olive Orchard. Agric. Water Manag. 2017, 191, 138–152. [Google Scholar] [CrossRef] [Scilit]
- Nadezhdina, N.; Vandegehuchte, M.W.; Steppe, K. Sap Flux Density Measurements Based on the Heat Field Deformation Method. Trees 2012, 26, 1439–1448. [Google Scholar] [CrossRef] [Scilit]
- Nadezhdina, N. Revisiting the Heat Field Deformation (HFD) Method for Measuring Sap Flow. iForest 2018, 11, 118. [Google Scholar] [CrossRef] [Scilit]
- Ferreira, M.I.; Conceição, N.; David, T.S.; Nadezhdina, N. Role of Lignotuber versus Roots in the Water Supply of Rainfed Olives. Acta Hortic. 2013, 991, 181–188. [Google Scholar] [CrossRef] [Scilit]
- Green, S.R.; Romero, R. Can We Improve Heat-Pulse to Measure Low and Reverse Flows. Acta Hortic. 2012, 951, 19–30. [Google Scholar] [CrossRef] [Scilit]
- Green, S.; Clothier, B.; Perie, E. A Re-Analysis of Heat Pulse Theory across a Wide Range of Sap Flows. Acta Hortic. 2009, 846, 95–104. [Google Scholar] [CrossRef] [Scilit]
- Siqueira, J.M.; Ferreira, M.I. Optimisation of CAG Technique: An Algorithm to Estimate Low and Reverse Sap Flow in Roots. Agric. For. Meteorol. 2020, 294, 108129. [Google Scholar] [CrossRef] [Scilit]
- Ferreira, M.I. Oliveira, a Antiga Arte de Não Morrer de Fome Nem de Sede: Estudos No Baixo Alentejo. In Proceedings of the VIII Simpósio Nacional de Olivicultura; SPH: Santarém, Portugal, 2020; p. 51. [Google Scholar]
- Lourenço, S.V.; Ferreira, M.I. Exploring Hydraulic Redistribution for Water Management in Gardens. Acta Hortic. 2020, 1279, 97–101. [Google Scholar] [CrossRef] [Scilit]
- Aganchich, B.; Wahbi, S.; Yaakoubi, A.; El-Aououad, H.; Bota, J. Effect of Arbuscular Mycorrhizal Fungi Inoculation on Growth and Physiology Performance of Olive Tree under Regulated Deficit Irrigation and Partial Rootzone Drying. S. Afr. J. Bot. 2022, 148, 1–10. [Google Scholar] [CrossRef] [Scilit]
- Polverigiani, S.; McCormack, M.L.; Eissenstat, D.M. Above-and below-Ground Responses to Soil Moisture Deficits in Olive. Acta Hortic. 2011, 888, 183–190. [Google Scholar] [CrossRef] [Scilit]
- Häusler, M.; Ferreira, M.I.; Conceição, N. Assessment of Vegetation Parameters in Olive Trees in the Region of Alentejo: A Comparison of Direct and Indirect Methods. Acta Hortic. 2014, 1038, 407–414. [Google Scholar] [CrossRef] [Scilit]
- Kottek, M.; Grieser, J.; Beck, C.; Rudolf, B.; Rubel, F. World Map of the Köppen-Geiger Climate Classification Updated. Meteorol. Z. 2006, 15, 259–263. [Google Scholar] [CrossRef] [Scilit]
- IPMA—Instituto Português do Mar e da Atmosfera. Boletim Meteorológico Para a Agricultura 1|13; IPMA: Lisbon, Portugal, 2019. [Google Scholar]
- Thomas, A.; Yadav, B.K.; Šimůnek, J. Root Water Uptake under Heterogeneous Soil Moisture Conditions: An Experimental Study for Unraveling Compensatory Root Water Uptake and Hydraulic Redistribution. Plant Soil 2020, 457, 421–435. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.