


Abstract
Seed germination and early root growth are decisive for crop establishment, yet responses to ionic environments can be strongly genotype-dependent. This study evaluated the effect of supplementing an agar-based in vitro system with a commercial NPK fertilizer on the germination dynamics and early seedling traits of Raphanus sativus L. Seeds were tested in two solid media: A (1.3% agar, no fertilizer) and AF (1.3% agar supplemented with 0.45 g of granular NPK fertilizer (15–30–15) per 200 mL medium), using a completely randomized 3 × 2 factorial design. Germination percentage and synchrony are key constituents of seedlot evaluation because they jointly capture both viability and the temporal coordination of emergence. However, final germination percentage alone does not reflect the timing and uniformity of germination, which can be critical for predicting establishment and subsequent performance. Therefore, indices such as mean germination time (MGT), coefficient of velocity of germination (CVG), and interval germination rates are frequently employed to describe germination dynamics. In addition to germination dynamics, early seedling morphometry (e.g., root and hypocotyl traits) can provide complementary information on early vigor and stress sensitivity under contrasting media or environmental conditions. Root elongation was significantly reduced by fertilization in ASD and GE, whereas AS exhibited consistently shorter roots with no significant response. PCA summarized 86.3% of the total variance in the first two components, separating treatments along a vigour/architecture axis and a germination capacity axis (%G), and hierarchical clustering identified five response groups. Overall, a low-cost agar + fertilizer system effectively discriminated genotype-specific sensitivity to an ionic environment during early establishment, highlighting the need to consider variety-dependent thresholds when using commercial fertilizers for in vitro screening.
1. Introduction
Seed germination and early seedling establishment represent a critical phase in the plant life cycle because they concentrate largely irreversible physiological decisions—metabolic reactivation, seed-cover weakening, radicle protrusion, and initial tissue differentiation—that ultimately shape seedling vigour and the probability of successful establishment. These processes are governed by the interplay between the internal status of the seed (developmental maturity, reserve mobilization capacity, membrane integrity, and dormancy level) and external drivers such as temperature, water availability, oxygen supply, and the ionic composition of the surrounding medium [1,2,3,4].
Among environmental drivers, the physicochemical properties of the germination medium—particularly its osmotic potential and ionic strength—strongly regulate water uptake, metabolic activation, and the rate and uniformity of germination [5]. Therefore, seed performance is typically evaluated not only by final germination but also by the speed and synchrony of emergence, which are closely related to subsequent establishment under practical conditions [6]. In addition, variation among commercial lots and varieties can be amplified by differences in seed ageing and survival, affecting both viability and early performance even before visible emergence occurs [7].
Although final germination percentage is widely used as a quality indicator, it is often insufficient to describe real seed lot performance: different treatments may reach similar final values but exhibit distinct temporal dynamics, translating into differences in synchrony, uniformity, and early vigour. For this reason, methodological frameworks emphasize quantifying the germination process as a time-dependent phenomenon rather than a single endpoint [8]. Likewise, critical evaluations of single-value germination indices show that the shape and dispersion of the cumulative curve contain biologically meaningful information that should be captured through complementary metrics [9]. This is consistent with the broader concept of seed vigour as the capacity to establish rapidly and uniformly, extending beyond mere viability [10].
Early growth—particularly the development of the primary root—constitutes another key component of vigour because it integrates reserve utilization efficiency, cell expansion, and the ability to explore the medium soon after emergence. Foundational plant physiology frameworks highlight that early root elongation is a sensitive readout of growth regulation and resource acquisition potential [11]. Because ionic and osmotic constraints can directly impair cell expansion and water relations, salinity tolerance mechanisms provide an explanatory framework for understanding how ionic stress conditions can penalize early establishment [12]. In parallel, mineral nutrition theory underscores that ions are essential to sustain metabolism and growth, yet imbalanced ionic environments can generate osmotic stress or ion-specific toxicity, compromising germination and seedling development [13,14].
In vitro systems provide a controlled platform to study these processes by minimizing environmental noise and enabling standardized comparisons across genotypes and treatments. Defined culture media have been central to plant tissue culture and early development research, with the Murashige–Skoog formulation serving as a widely adopted reference for controlled growth [15]. Comprehensive tissue culture manuals further emphasize the importance of medium composition and physical support matrices for reproducible development [16]. At the same time, low-cost approaches—including alternative gelling agents and simplified support matrices—have been explored to facilitate large-scale or resource-limited experimentation [17]. However, the interpretability of in vitro assays depends strongly on asepsis: contamination can rapidly alter local pH, oxygen availability, and nutrient dynamics, biasing treatment effects [18], and microbial hazards remain a recurrent challenge in plant tissue and cell culture systems [19].
Accordingly, robust surface-sterilization and establishment protocols are essential to ensure that observed differences reflect treatment and genotype rather than uncontrolled microbial growth. Recent work has demonstrated that optimization of in vitro sterilization and germination conditions benefits from systematic modeling and predictive approaches [20]. From a design standpoint, factorial experiments are especially valuable because they allow separation of main effects (e.g., genotype and fertilization) and their interaction under randomized conditions [21]. When multiple treatments are compared, classical multiple-comparison procedures remain standard for mean separation after ANOVA [22], while rank-based nonparametric approaches provide alternatives when normality assumptions are not met [23,24]. Moreover, controlling error rates under multiple testing is critical to preserve inferential validity, particularly when several indices and response variables are analyzed simultaneously [25].
Beyond univariate inference, early establishment is increasingly interpreted as a multivariate phenotype in which germination dynamics and growth traits covary. Multivariate exploratory tools such as principal component analysis (PCA) and hierarchical clustering can complement univariate tests by summarizing correlated germination and morphometric traits and highlighting treatment groupings [26,27]. Accordingly, we used PCA and clustering to visualize the joint response of radish varieties to contrasting ionic environments [28,29].
Radish (Raphanus sativus L.) is frequently used as a rapid and informative model for germination and early growth studies due to its short emergence time and sensitivity to metabolic and environmental modulation, making it well suited for detecting genotype-dependent responses under controlled conditions [30]. To ensure comparability and reproducibility, seed testing standards recommend rigorous sampling procedures and controlled handling, which are particularly relevant when working with commercial seed lots [31]. In addition, reproducible statistical workflows benefit from validated software ecosystems: multivariate analyses are commonly implemented with dedicated R packages for PCA and related methods [32], complemented by visualization tools for extracting and communicating multivariate results [33], all within the R statistical computing environment [34].
Mechanistic and semi-mechanistic modeling further strengthens interpretation of germination dynamics by explicitly linking rate processes to water relations and temperature constraints. Fertilizer addition increases ionic strength and can reduce the effective water potential of the germination medium, creating osmotic and ionic constraints that delay imbibition and radicle protrusion. Therefore, we expected fertilizer-supplemented media to modify germination speed and synchrony, with responses differing among varieties [35,36,37,38,39,40,41,42].
Complementary to modeling, classical indices remain valuable for practical discrimination among treatments and seed lots when applied with appropriate caution. Indices combining speed and completeness, such as germination value, have long been used to integrate performance dimensions into single interpretable measures [43,44]. Moreover, frequent radicle-emergence scoring has been shown to improve the predictive value of time-based metrics for seed vigour, reinforcing the importance of high-resolution temporal data in early establishment studies [45].
In this work, we used three widely cultivated commercial radish (Raphanus sativus L.) varieties (Cherry Belle, Sparkler, and Daikon) as contrasting genotypes to test whether fertilizer addition to the germination medium (agar-only vs. agar + NPK) alters germination dynamics and early seedling traits through changes in ionic strength, and whether these responses are variety-dependent. Beyond describing experimental effects, the practical goal is to inform seedlot screening and nursery/propagation management by identifying varieties (or lots) that are more sensitive to high-ionic-strength germination conditions.
This approach provides a rapid, controlled framework to compare early-stage sensitivity to fertilizer-induced ionic environments, which can be used as a practical screening step before greenhouse or field establishment.
2. Materials and Methods
2.1. Plant Material and Experimental Conditions
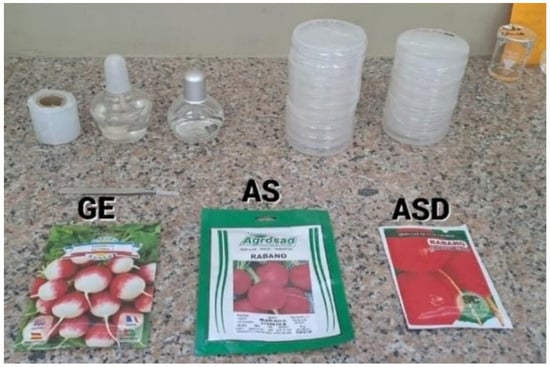
A completely randomized 3 × 2 factorial design was used, with Variety (Cherry Belle, Sparkler, and Daikon) and Medium (A, agar-only; AF, agar + fertilizer) as fixed factors (Figure 1). For germination and root-length traits, each Petri dish containing nine surface-sterilized seeds was considered one experimental unit; three independent dishes were prepared per treatment combination (n = 3), yielding 18 dishes in total. For seedling morphometry, all germinated seedlings per dish (up to 9 seedlings) were measured at 72 h, and their measurements were averaged per dish so that the dish remained the experimental unit for statistical analyses.
Figure 1.
Seeds of Agrosad (AS), Agrícola Santo Domingo (ASD), and Garden Elite (GE).
2.2. Experimental Design
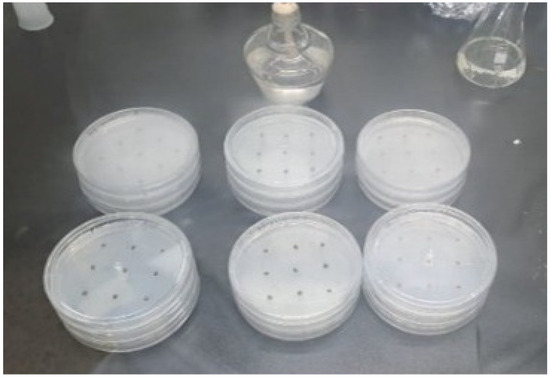
The experiment was conducted under a completely randomized design (CRD) with a 3 × 2 factorial arrangement, allowing estimation of the main effects of Variety and Fertilization and their interaction through random allocation of experimental units [21]. The design structure and the definition of experimental units by response variable are summarized in Table 1 and Table 2, and the sowing layout is illustrated in Figure 2.
Table 1.
Structure of the 3 × 2 factorial design (CRD).
Table 2.
Experimental units, replication, and sample sizes by response variable.
Figure 2.
Seed sowing arrangement in a 3 × 3 grid.
2.3. Treatments
Two solid media were prepared to generate contrasting ionic environments: (i) A (agar-only), consisting of 1.3% (w/v) agar dissolved in distilled water; and (ii) AF (agar + fertilizer), consisting of 1.3% (w/v) agar supplemented with 0.45 g of granular NPK fertilizer (15–30–15) per 200 mL medium. Prior to sowing, seeds were surface-disinfected by immersion in 2% sodium hypochlorite for 10 min, rinsed three times with sterile distilled water, and air-dried under sterile conditions. Plates were sealed with Parafilm and incubated at 25 ± 2 °C in darkness [17,20].
2.4. Assessments and Measured Variables
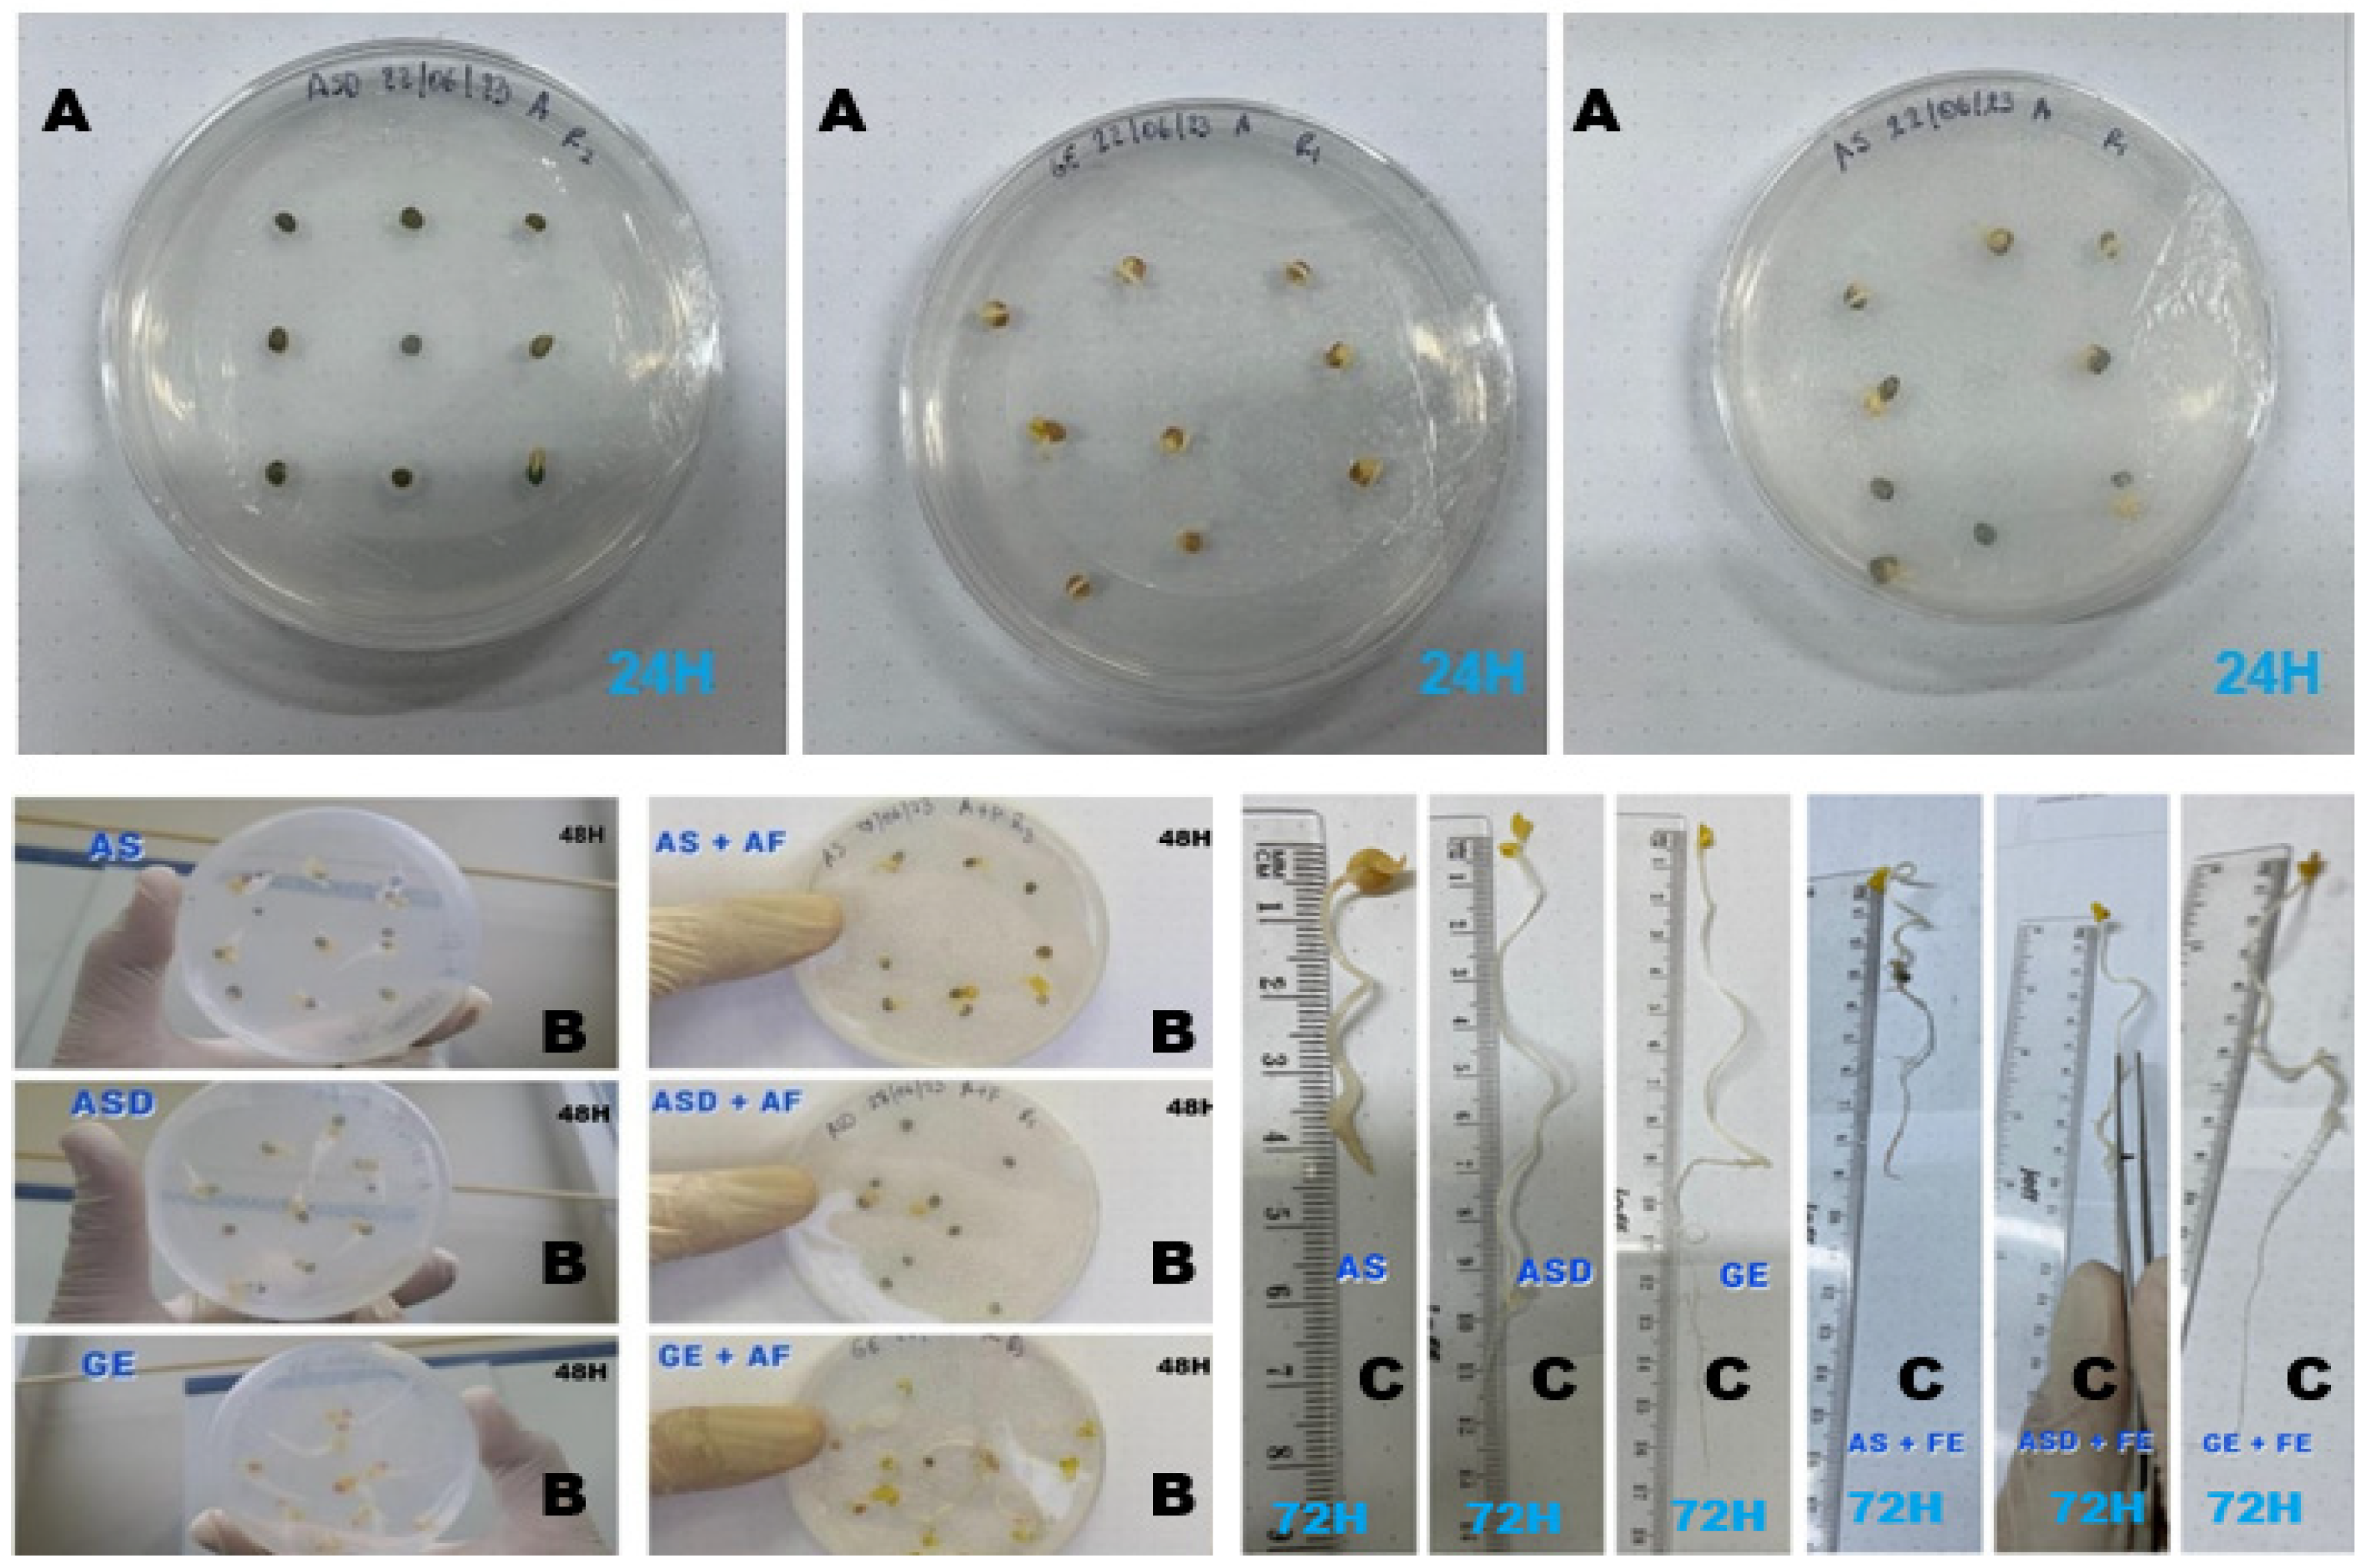
Interval germination was recorded per replicate at 24, 48, and 72 h as the number of newly germinated seeds in each interval: G24 = n0–24, G48 = n24–48, and G72 = n48–72 (where n denotes the count of newly germinated seeds in the specified interval). For clarity, G24–G72 represent interval counts (not cumulative germination percentage); cumulative germination (%) was reported separately as the proportion of germinated seeds relative to the total number of seeds per plate (N = 9) (Figure 3).
Figure 3.
Germination was recorded at 24 (A), 48 (B), and 72 (C) h of incubation. After 72 h, representative seedlings of each variety were photographed to illustrate differences in early root elongation under the evaluated conditions.
2.4.1. Primary Variables
Interval germination (G24, G48, G72) was defined as the number of seeds germinated within each evaluation period: G24 (0–24 h), G48 (24–48 h), and G72 (48–72 h). This interval-based approach characterizes emergence dynamics and discriminates treatments that may reach similar final germination but at different rates.
Root length (72 h) was defined as the length (cm) of the primary root measured at 72 h. For each plate, all germinated seedlings were measured and the plate-level mean root length was used as the experimental unit for statistical analysis. This approach yielded three replicate observations per treatment (18 plates in total) while accommodating treatment-dependent differences in germination.
2.4.2. Calculated Germination-Performance Indices
From interval germination counts, standard germination-performance indices were calculated as follows (N = 9 seeds per plate):
Final germination percentage (%G):
where is the total number of germinated seeds accumulated up to 72 h .
Mean germination time (MGT): computed following Ellis and Roberts [7]:
Lower values indicate faster average germination.
Germination speed index (IVG): computed following Maguire [6]. To match the evaluation frequency, time was expressed in days equivalent to 24, 48, and 72 h ():
Higher values indicate greater vigour due to earlier and more concentrated emergence.
Coefficient of velocity of germination (CVG): computed following Kotowski [5]:
where is expressed in hours. Higher values indicate faster germination.
2.5. Statistical Analysis
To ensure traceability between each response variable and the inferential method applied, the statistical approach is summarized in Table 3. Statistical significance was set at α = 0.05 for all tests, and multiple-comparison or p-value adjustment procedures were applied when appropriate to control multiplicity [21,25].
Table 3.
Summary of statistical analyses by variable.
Specifically, plate-level germination variables (%G, IVG, CVG) were analyzed using a 3 × 2 factorial ANOVA with three replicates per treatment under a completely randomized design [21]. When significant effects were detected (), Tukey’s HSD test was used for mean separation [22]. Because germination and seedling traits are partially correlated, we first applied a two-way MANOVA (Variety, Medium, and their interaction) to test for an overall multivariate treatment effect across the response vector [24,25]. When the MANOVA indicated significant effects, we conducted follow-up two-way ANOVAs for each trait to identify which variables contributed to the multivariate signal [21]. Normality and homoscedasticity were assessed using Shapiro–Wilk and Levene’s tests; when needed, data were transformed prior to inference. Post hoc comparisons were performed using Tukey’s HSD at α = 0.05. Given the replication level (n = 3 dishes per treatment), results were interpreted with emphasis on effect magnitude and consistency across traits. Analyses were conducted in JMP Pro 16 [28,29]. As a limitation, the design uses three replicates per treatment, which may reduce statistical power for small effects; therefore, non-significant outcomes are interpreted cautiously and discussed in light of biological plausibility and multivariate patterns.
2.6. Software
All analyses were performed in the R statistical computing environment (version 4.2.1) [34]. ANOVA models, Kruskal–Wallis and Wilcoxon tests, and Tukey multiple comparisons were implemented using base R functions. PCA and hierarchical clustering workflows were conducted using FactoMineR (version 2.12) [32], and results extraction and visualization (biplots and dendrograms) were produced with factoextra [33]. Statistical significance was set at α = 0.05 for all inferential procedures.
3. Results
3.1. Effect of Fertilization on Germination and Morphometry of Raphanus sativus L.
To determine the overall treatment effect, a MANOVA using Pillai’s trace was performed. Results showed highly significant differences for both Variety (Pillai = 1.73; p < 0.001) and Fertilization (Pillai = 0.80; p < 0.001), as well as for their interaction (V × F; Pillai = 1.18; p < 0.01).
Univariate ANOVAs confirmed these patterns for most variables, whereas for MGT the nonparametric analysis also indicated significant differences. Variety was the most influential source of variation, particularly for IVG, which showed the highest F value (F = 169.82; p < 0.001). Importantly, the V × F interaction was significant across all parameters, demonstrating that the response to fertilization was not uniform but genotype-dependent. Statistical details are summarized in Table 4.
Table 4.
Summary of univariate (ANOVA) and multivariate (MANOVA) analyses evaluating genotype and ionic-environment effects.
Mean comparisons (Table 5) decomposed the interaction patterns. For final germination (%G), varieties AS and GE were stable, with no statistical differences between control and fertilized treatments, maintaining values above 88%. In contrast, ASD showed a severe negative impact under fertilization, dropping from 88.89% (control) to 25.93% (fertilized).
Table 5.
Differences in germination and early seedling traits among radish varieties under agar-only (A) and agar + fertilizer (AF) media. Values are means ± SD (n = 3 plates per treatment).
Regarding speed and development, fertilization tended to delay germination, evidenced by a significant increase in MGT for AS and GE, and a generalized reduction in IVG, with ASD again being the most affected (lowest value in the experiment: 1.23). Root development was strongly inhibited by fertilization in ASD and GE, both showing significant reductions compared to their controls (from 9.15 cm and 9.40 cm down to 5.20 cm and 4.00 cm, respectively). Notably, GE reduced its root length to less than half. By contrast, AS presented the shortest root length in both conditions, with no significant change due to fertilization.
3.2. Association Patterns Among Variables and Treatment Classification
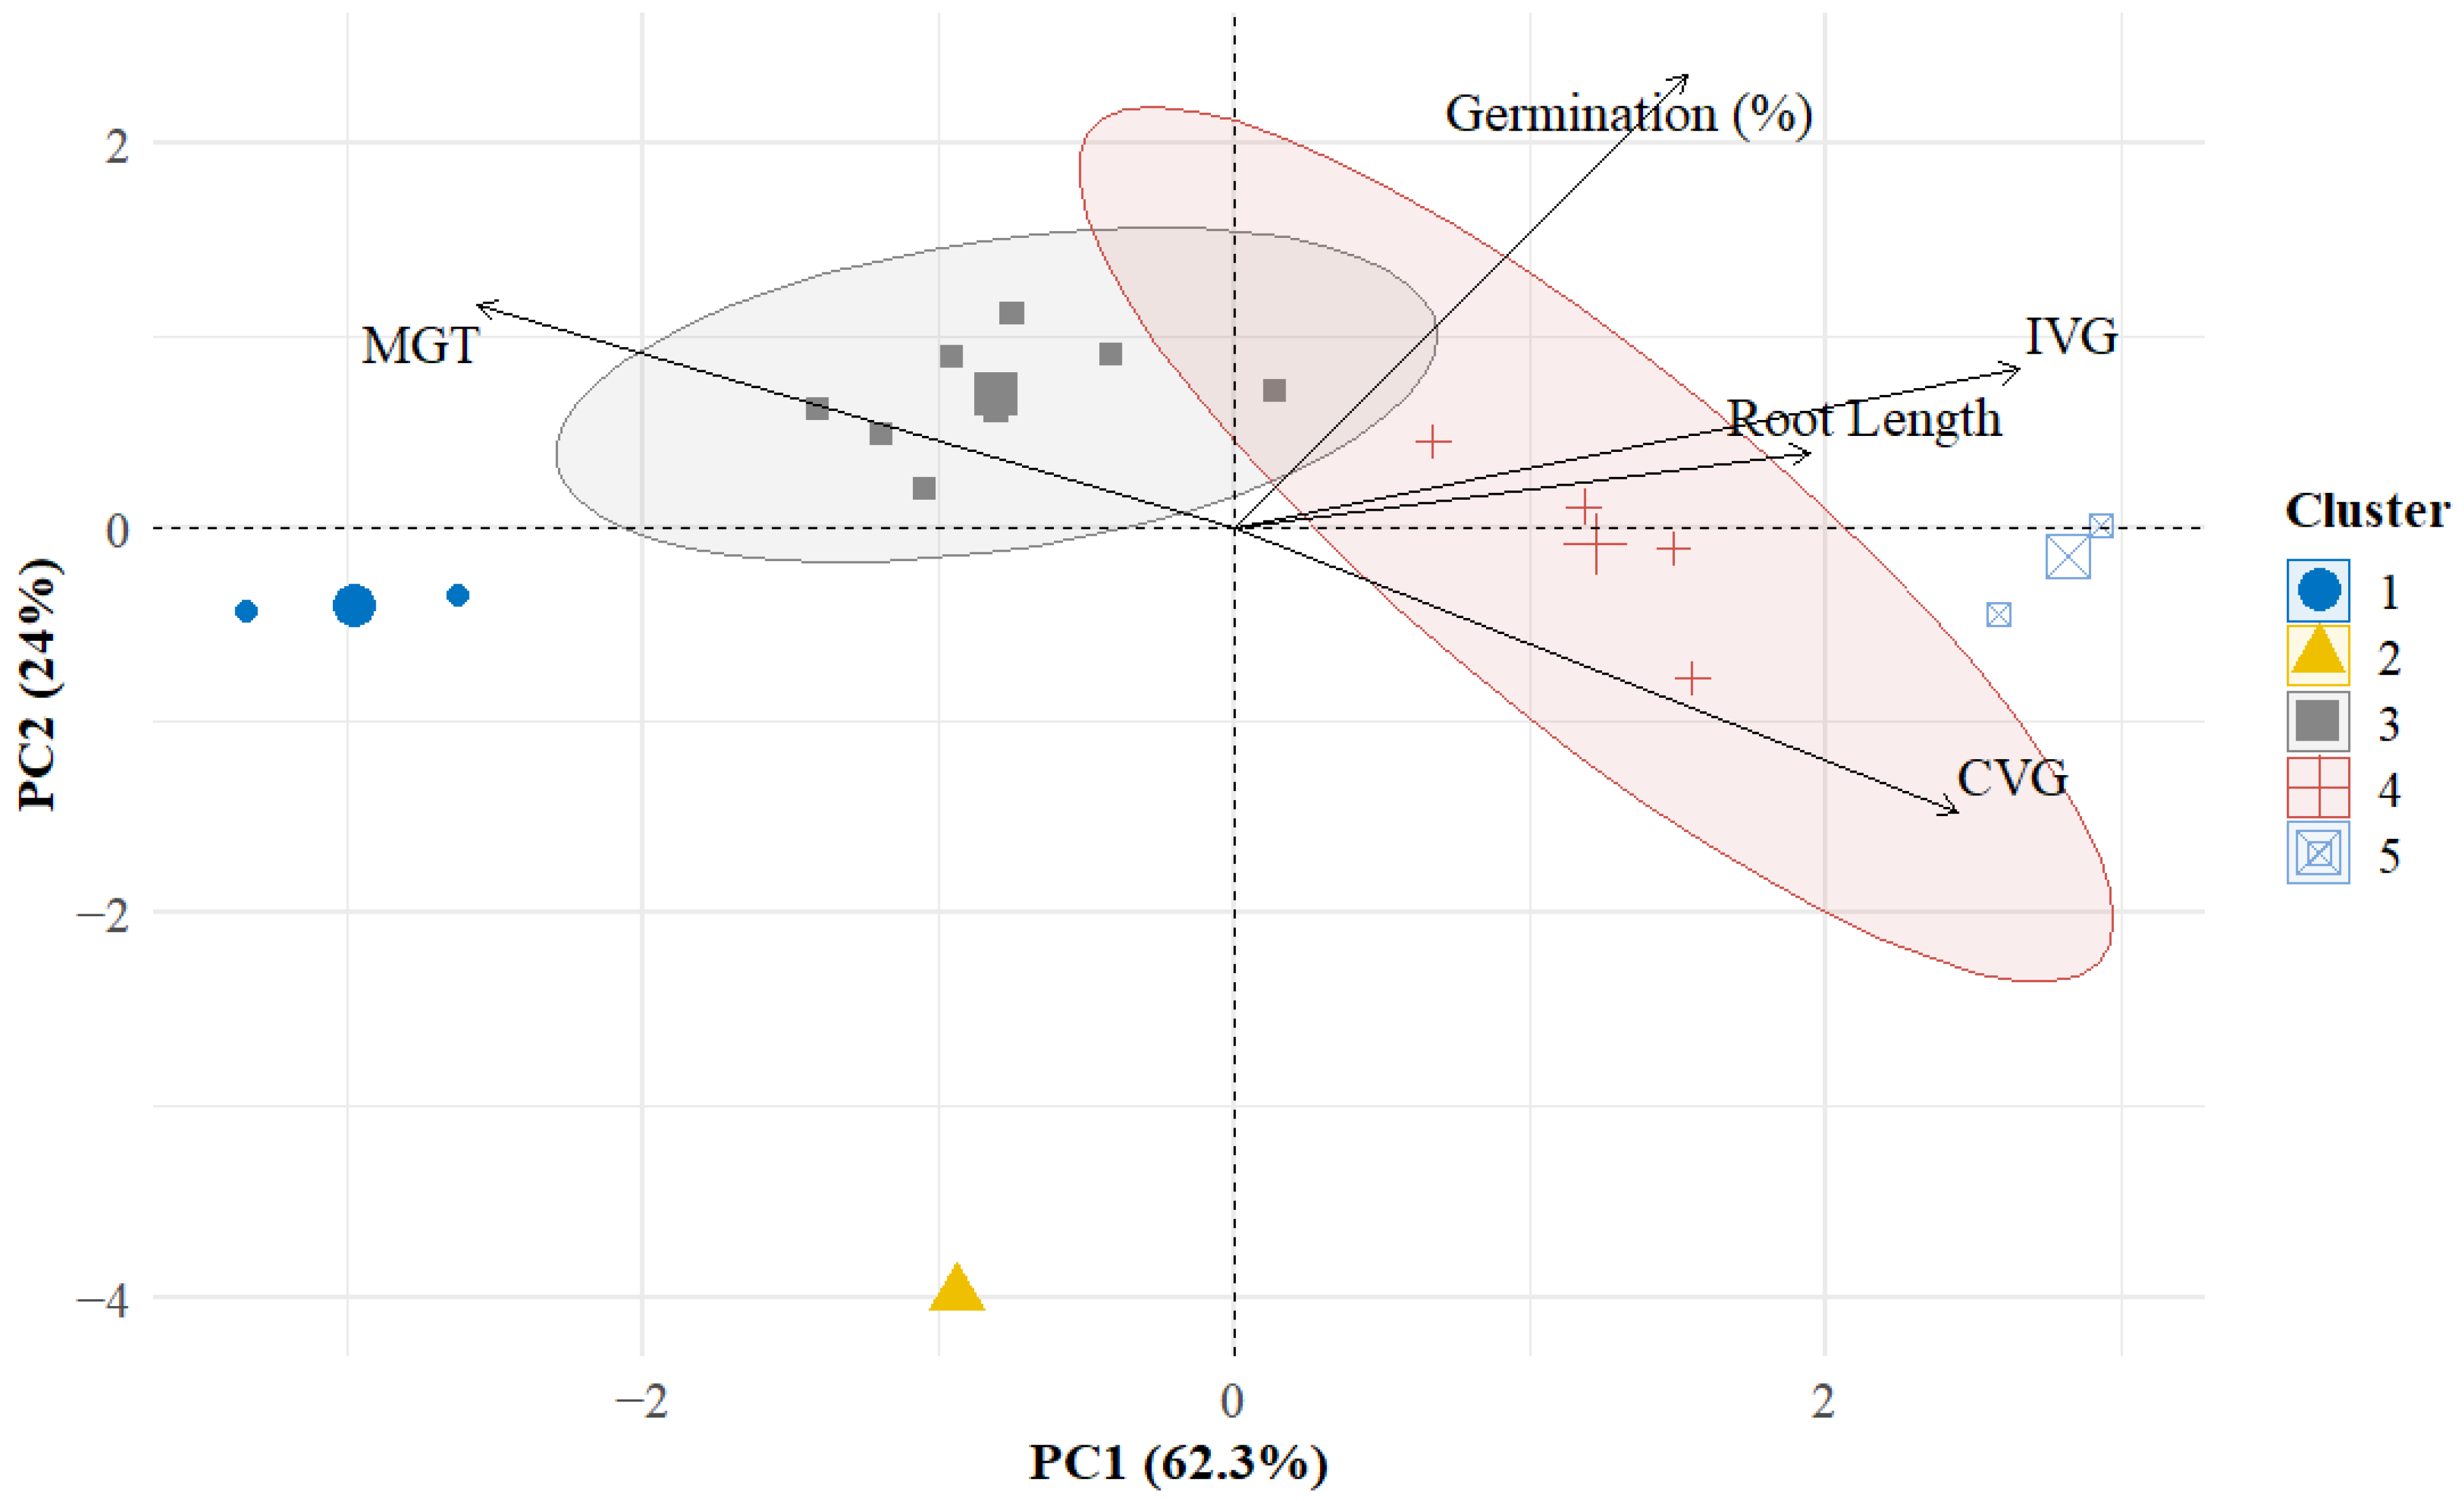
To understand the structure of relationships among variables and to classify treatments based on overall response, a PCA was performed. PCA is explicitly intended for sets of inter-correlated quantitative variables; therefore, correlation among germination indices (e.g., MGT and CVG) does not invalidate the explained-variance percentages, which are derived from the eigen-decomposition of the (standardized) correlation/covariance structure. In this context, highly correlated indices are expected to align with the same latent germination-speed dimension, and interpretation is therefore based on the loading pattern rather than on the number of correlated indicators [46]. Principal component analysis (PCA) revealed that the first two components explained 86.3% of the total variance (PC1 = 62.3%, PC2 = 24%; Figure 4). The biplot indicated that IVG, germination (%), cotyledon width, and cotyledon length contributed most to the separation along PC1, whereas MGT and hypocotyl length loaded more strongly on PC2.
Figure 4.
Principal component analysis (PCA) biplot of plate-level responses (n = 18; 3 varieties × 2 media × 3 replicates) based on standardized germination-performance and early seedling-growth variables: final germination percentage (%G, %), mean germination time (MGT, h), germination speed index (IVG, index), coefficient of velocity of germination (CVG, %), and root length at 72 h (cm). MGT and CVG does not compromise the explained-variance percentages, but indicates shared germination-speed information. Points represent individual plate observations, symbols/colors indicate HCPC cluster membership, and vectors indicate variable loadings in the PCA space. PCA scores are dimensionless because variables were z-standardized before analysis. PC1 and PC2 explained 62.3% and 24.0% of the total variance, respectively. Symbol/color coding indicates HCPC clusters: Cluster 1 (blue circles), Cluster 2 (yellow triangles), Cluster 3 (gray squares), Cluster 4 (red crosses), and Cluster 5 (light-blue squares).
Projection of treatments in the biplot (Figure 4) revealed fertilization-driven dispersion. Variety AS showed high phenotypic stability, with both control and fertilized treatments positioned close to each other and associated with high vigour (positive PC1). In contrast, fertilization produced a pronounced separation in ASD, shifting fertilized samples toward the negative quadrant for both vigour and germination, far from their respective controls.
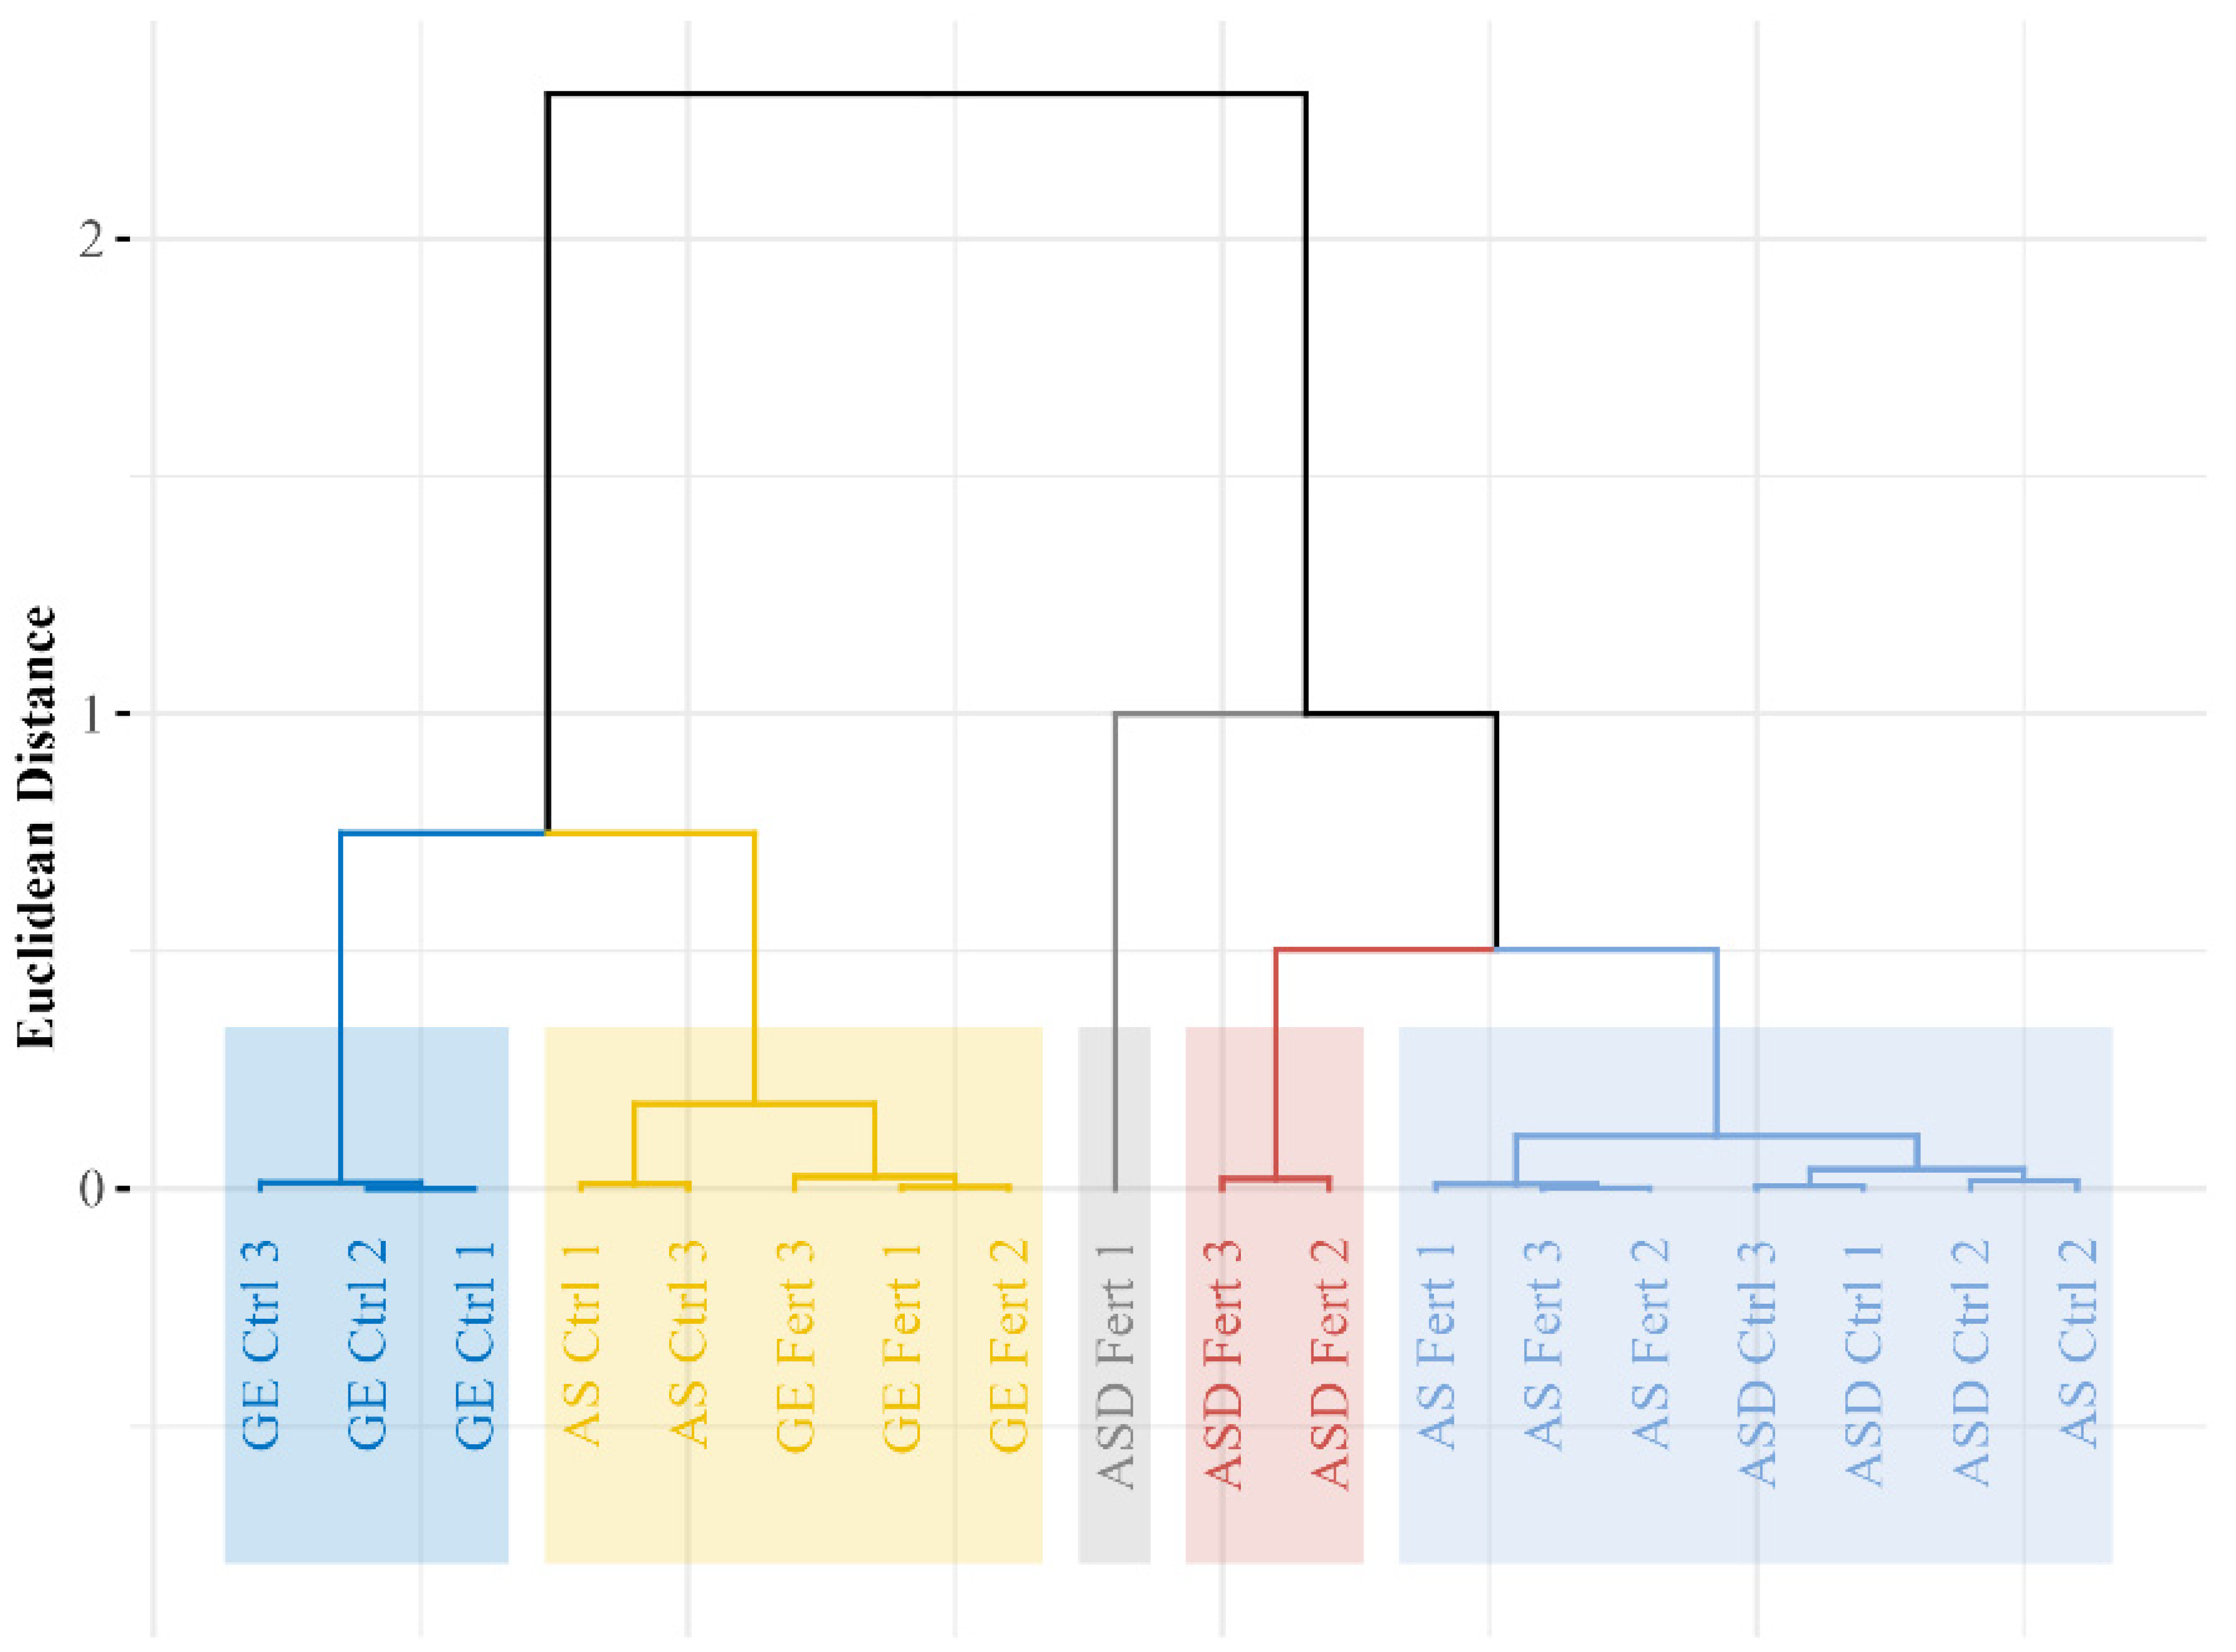
This pattern was corroborated and formally classified by hierarchical clustering (Figure 5), which identified five groups with distinct behaviors. ASD controls clustered with the best-performing treatments (light-blue cluster), whereas fertilization segregated ASD-Fert into an independent group (red/gray clusters) characterized by low global performance. Additionally, GE (Control) formed an isolated group (dark-blue cluster), clearly differentiated from its fertilized counterpart due to moderate speed and root length.
Figure 5.
Hierarchical clustering dendrogram of evaluated treatments. Treatment labels follow the format Variety–Medium–Replicate, where AS = Sparkler, ASD = Daikon, and GE = Cherry Belle; A = agar-only and AF = agar + fertilizer; and Replicate denotes the Petri-dish replicate (1–3). Colored background blocks indicate the five clusters identified by hierarchical clustering (dark blue, yellow, gray, red, and light blue).
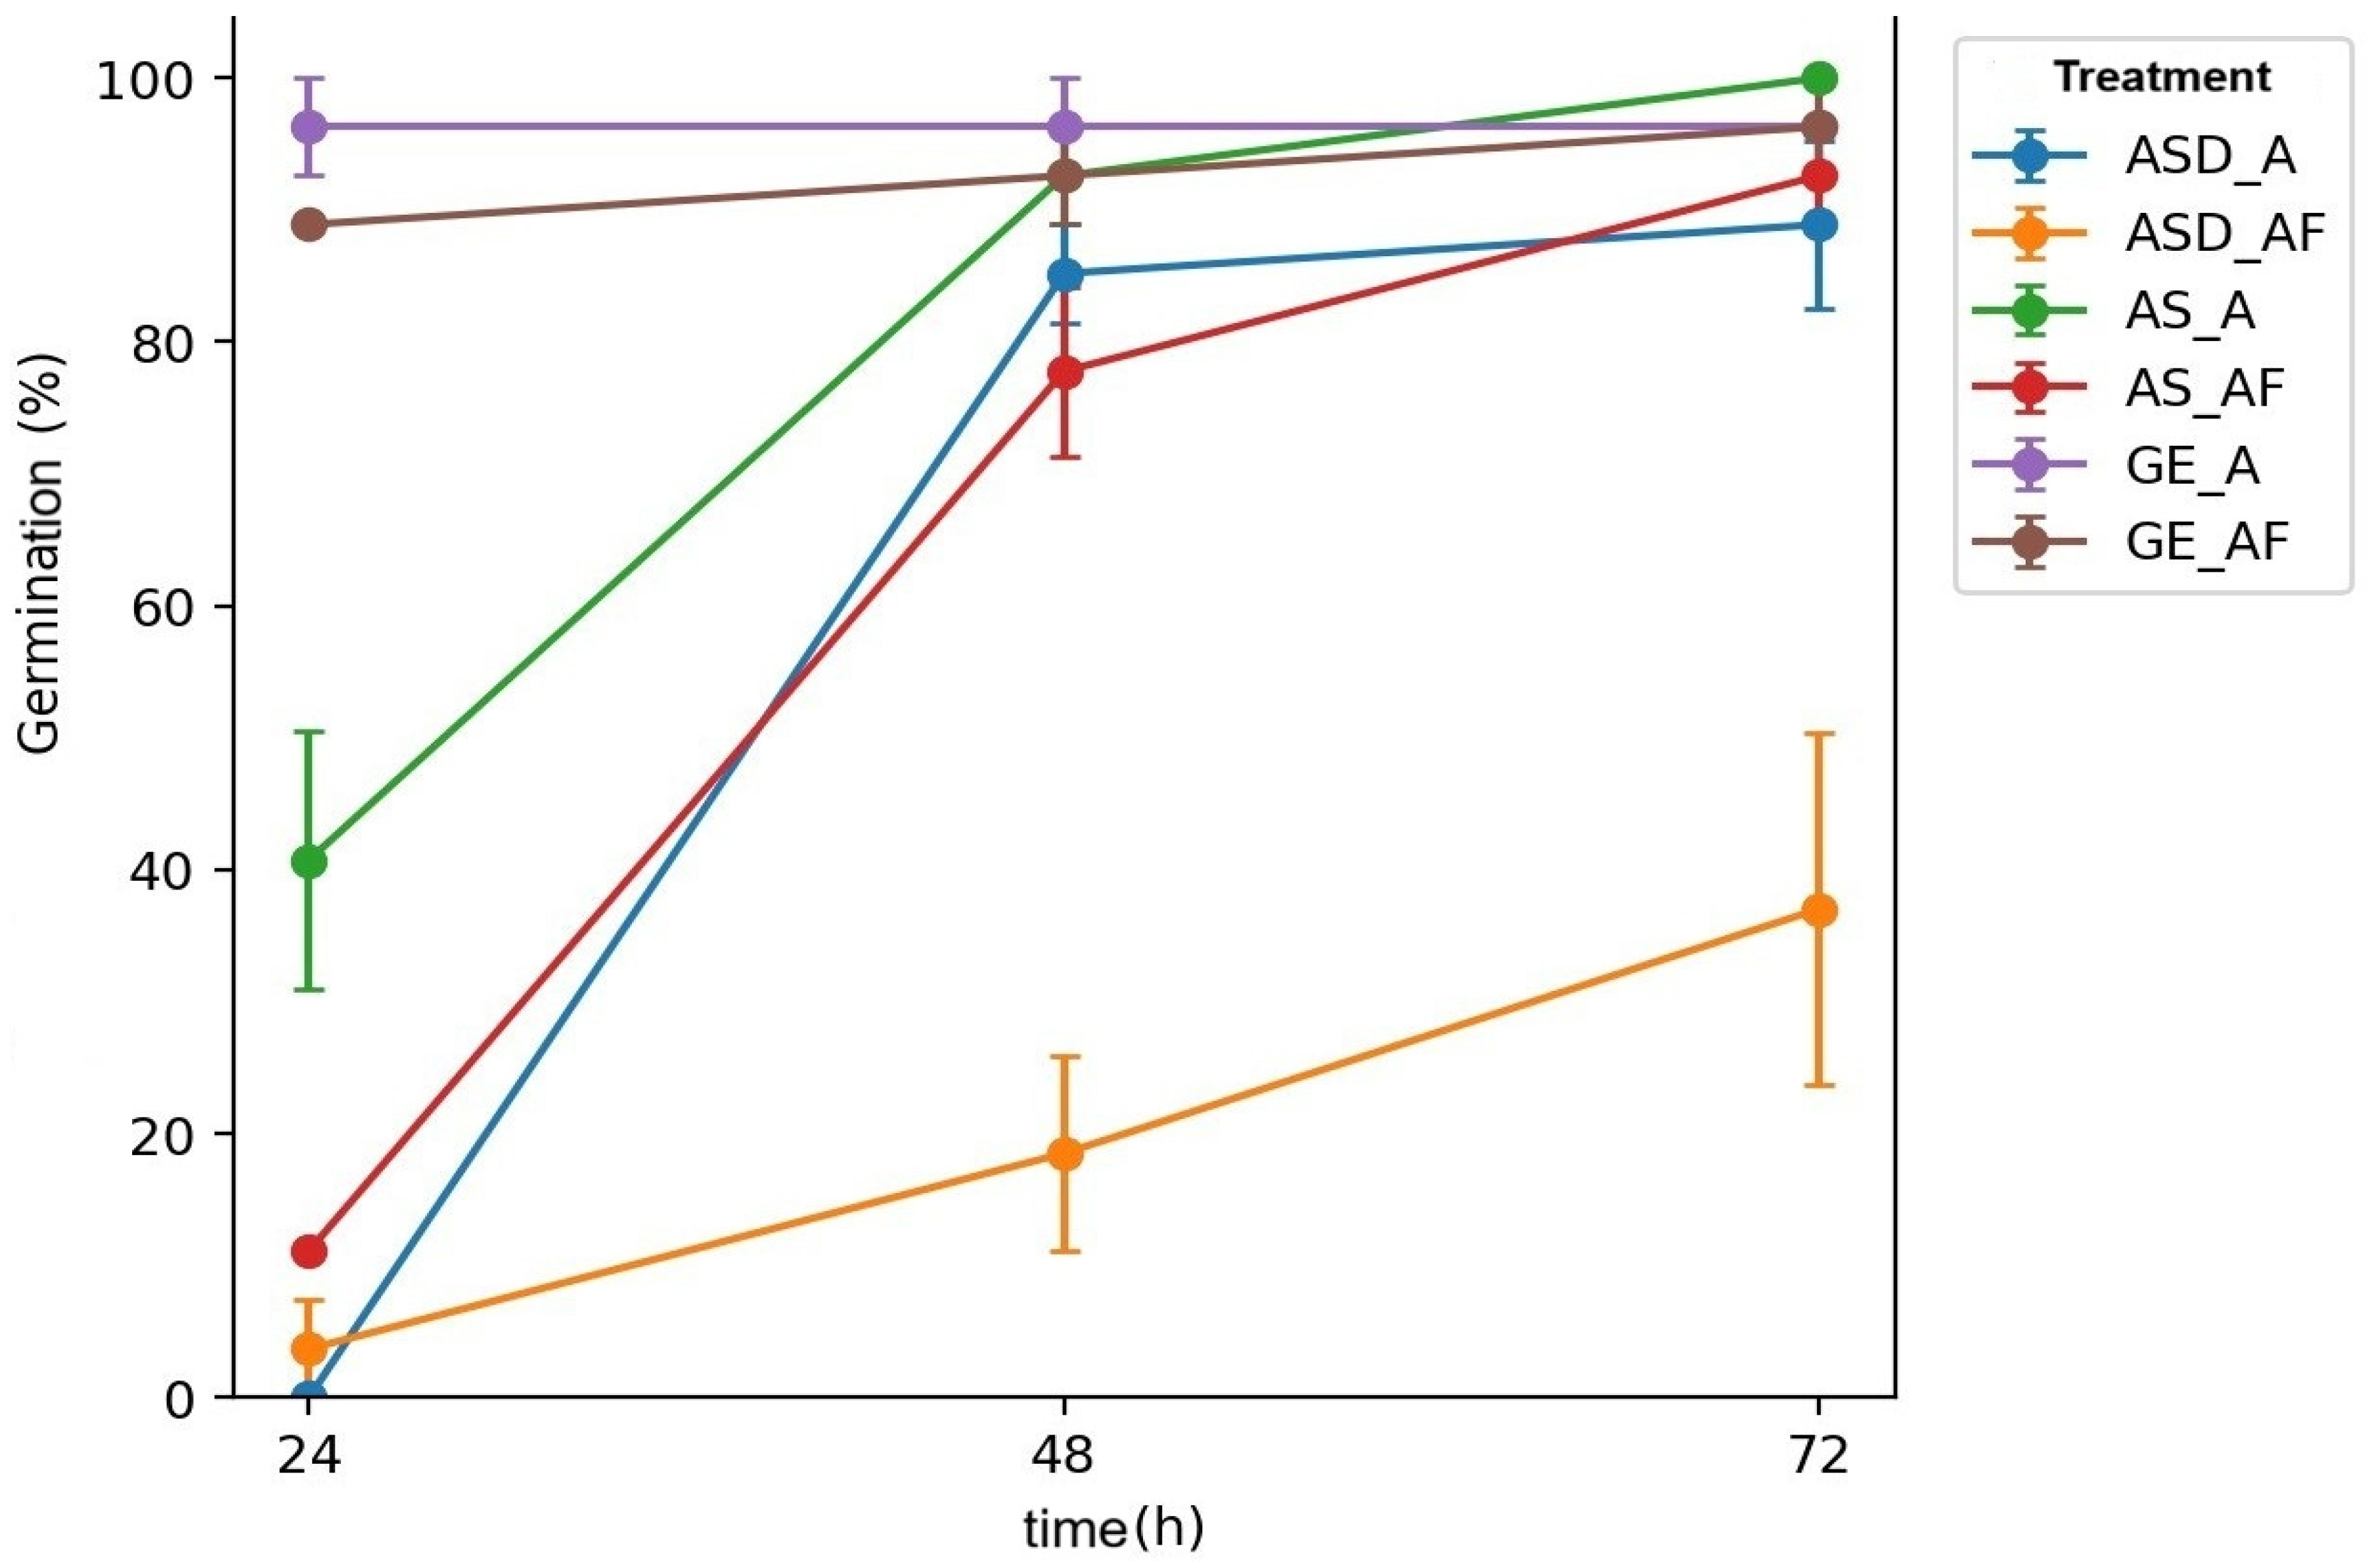
Finally, Figure 6 shows a differential response in cumulative germination driven by the Variety × Fertilization interaction. The imported variety GE showed the fastest establishment, reaching near-maximum values by 24 h in medium A (GE_A) and remaining nearly stable up to 72 h, whereas GE_AF began slightly lower but converged to high final percentages. In contrast, domestic materials showed greater medium dependence: AS_A increased markedly between 24 and 48 h and achieved the highest final germination at 72 h, while AS_AF exhibited an initial delay but partially recovered by 72 h. The strongest fertilization effect was observed in ASD, where ASD_AF maintained low germination throughout the assay with higher variability (SE), suggesting an inhibitory effect of mineral supplementation on early emergence in this genotype, unlike ASD_A, which increased rapidly between 24 and 48 h and stabilized thereafter.
Figure 6.
Cumulative germination dynamics by treatment (mean ± SE).
4. Discussion
The strong Variety × Fertilization interaction observed in this experiment (notably the collapse of %G and IVG in ASD under AF, together with the marked inhibition of root elongation in ASD and GE) indicates that adding a commercial NPK blend to an agar-based in vitro system acts less as a “universal nutrient boost” and more as a genotype-specific ionic/osmotic filter, where small differences in seed physiology, membrane integrity, reserve mobilization, and ion-handling capacity are amplified under controlled conditions.
A plausible interpretation for the observed delays in germination and reductions in early root length under the fertilizer-supplemented medium is that the AF treatment altered the physicochemical environment of the medium (e.g., solute concentration/osmotic conditions), which may have slowed early emergence and elongation in some genotypes [47,48,49,50,51]. However, because this study measured germination dynamics and plate-level root length only, these results should be interpreted as early phenotypic responses rather than direct evidence of specific physiological mechanisms (e.g., osmotic stress, nutrient toxicity, or improved nutrition). The stronger AF-associated root-length reductions observed in ASD and GE, compared with AS, support a genotype-dependent response to the tested in vitro media conditions [52,53,54]. Such early-stage sensitivity is consistent with reports that newly emerged seedlings may show delayed growth or reduced vigor under elevated solute concentrations, even when nutrients are present [55].
The fact that GE exhibited rapid establishment in the control yet lost more than half of its root length under AF also fits a stress-response pattern reported in microgreen/brassicaceous systems under combined thermal/ionic constraints highlighting the importance of jointly interpreting germination curves and morphometry instead of relying on %G alone [56]. Statistically, the study’s multi-endpoint structure (several vigor indices + morphology + multivariate profiling) strengthens inference when multiplicity is explicitly controlled, and future expansions with finer temporal scoring or additional traits should consider procedures robust to dependency among tests (common in correlated vigor variables), such as FDR control under dependency and/or sequentially rejective adjustments to keep conclusions stable as the number of outcomes increases [57,58].
The genotype-dependent patterns observed here are consistent with integrated genotype × medium effects during early establishment. However, mechanistic explanations involving nitrate signaling, ROS dynamics, or hormonal regulation remain hypotheses in the context of this study, because no physiological or biochemical measurements were collected. Therefore, the present results are best interpreted as a screening-level phenotypic contrast among varieties under two defined in vitro media conditions, with clear differences in germination dynamics and early root elongation [59,60,61,62,63,64,65,66,67,68,69,70,71].
Methodologically, these findings support treating commercial fertilizer–agar systems as a low-cost screening tool rather than as a replacement for defined media: classic culture-medium research emphasizes that mineral requirements and ion forms matter, and micropropagation literature shows that “commercially feasible” protocols often succeed by controlling specific medium components and interactions rather than by increasing generic fertilization; thus, a rational next step is to chemically characterize AF (EC, pH, major ion forms, N speciation) and run a small concentration series to identify thresholds where each genotype transitions from stimulation to inhibition [59,60]. In parallel, complementary pre-sowing strategies—such as priming and targeted seed treatments known to improve emergence and early growth under abiotic stress—could be tested as practical countermeasures to AF-induced inhibition, especially for ASD-like sensitive lots [61,62,63].
Overall, multivariate profiling complemented the univariate results by separating treatments primarily by medium and secondarily by variety (Figure 4), reinforcing the interpretation that medium conditions were a dominant driver of early response patterns [72,73].
5. Conclusions
This study demonstrates that supplementing an agar-based in vitro system with a commercial NPK fertilizer (0.45 g per 200 mL medium; AF treatment) produces a strong genotype-dependent response during early establishment of Raphanus sativus L. The significant Variety × Fertilization interaction confirms that fertilization effects cannot be generalized across materials: while AS and GE maintained high final germination, fertilization tended to delay germination and reduce vigor, and it strongly inhibited root elongation in GE. The national variety ASD exhibited the greatest sensitivity, showing a drastic reduction in germination and the lowest vigor under fertilization, indicating that the fertilizer-generated ionic environment can act as an inhibitory filter for specific genotypes. Multivariate profiling (PCA and hierarchical clustering) integrated germination and growth traits, separating treatments along axes of vigor/architecture and germinative capacity, and consistently classifying treatments into distinct response groups, thereby strengthening interpretation beyond single variables. Overall, a low-cost agar + fertilizer assay is a practical approach to rapidly screen varietal sensitivity to ionic environments, but its use should be supported by dose–response testing and characterization of the medium (e.g., EC/pH and ion forms) to define safe thresholds and improve reproducibility across genotypes and seed lots.
Author Contributions
Conceptualization, L.C.-M., K.R.-P., J.F.G.-V., B.P.-G., S.V.-A., R.P.-P., I.A.A.G., E.R.-N. and C.E.D.E.; methodology, L.C.-M., K.R.-P., B.P.-G., R.P.-P., S.P.J.J., E.R.-N. and C.E.D.E.; software, I.I.-V., S.V.-A. and I.A.A.G.; validation, I.I.-V., S.V.-A. and I.A.A.G.; formal analysis, L.C.-M., J.F.G.-V., I.I.-V. and S.V.-A.; investigation, L.C.-M., K.R.-P., J.F.G.-V., B.P.-G., S.V.-A. and E.R.-N.; resources, L.C.-M., J.F.G.-V., S.P.J.J. and C.E.D.E.; data curation, I.I.-V. and S.V.-A.; writing—original draft preparation, L.C.-M. and C.E.D.E.; writing—review and editing, L.C.-M., K.R.-P., B.P.-G., I.I.-V., S.V.-A., R.P.-P., S.P.J.J. and E.R.-N.; visualization, L.C.-M., K.R.-P., B.P.-G., R.P.-P., I.A.A.G., E.R.-N. and C.E.D.E.; supervision, L.C.-M., E.R.-N. and C.E.D.E.; project administration, C.E.D.E. All authors have read and agreed to the published version of the manuscript.
Funding
This research received no external funding.
Data Availability Statement
The original contributions presented in this study are included in the article. Further inquiries can be directed to the corresponding author.
Acknowledgments
The authors are grateful to the Universidad Estatal de Milagro (UNEMI) for supporting our publication.
Conflicts of Interest
Author Ivana Alexandra Armijos Galarza is employed by Argroinisumos Fertisa Favorita. The remaining authors declare that the research was conducted in the absence of any commercial or financial relationships that could be construed as a potential conflict of interest.
References
- Baskin, C.C.; Baskin, J.M. Seeds: Ecology, Biogeography, and Evolution of Dormancy and Germination, 2nd ed.; Academic Press: San Diego, CA, USA, 2014. [Google Scholar]
- Bewley, J.D.; Bradford, K.J.; Hilhorst, H.W.M.; Nonogaki, H. Seeds: Physiology of Development, Germination and Dormancy, 3rd ed.; Springer: New York, NY, USA, 2013. [Google Scholar]
- Nonogaki, H.; Bassel, G.W.; Bewley, J.D. Germination—Still a mystery. Plant Sci. 2010, 179, 574–581. [Google Scholar] [CrossRef] [Scilit]
- Copeland, L.O.; McDonald, M.B. Principles of Seed Science and Technology, 4th ed.; Springer/Kluwer Academic: New York, NY, USA, 2001. [Google Scholar] [CrossRef] [Scilit]
- Kotowski, F. Temperature relations to germination of vegetable seed. Proc. Am. Soc. Hortic. Sci. 1926, 23, 176–184. [Google Scholar]
- Maguire, J.D. Speed of germination—Aid in selection and evaluation for seedling emergence and vigor. Crop Sci. 1962, 2, 176–177. [Google Scholar] [CrossRef] [Scilit]
- Ellis, R.H.; Roberts, E.H. The quantification of ageing and survival in orthodox seeds. Seed Sci. Technol. 1981, 9, 373–409. [Google Scholar]
- Ranal, M.A.; Santana, D.G. How and why to measure the germination process? Rev. Bras. Bot. 2006, 29, 1–11. [Google Scholar] [CrossRef] [Scilit]
- Brown, R.F.; Mayer, D.G. Representing cumulative germination: A critical analysis of single-value germination indices. Ann. Bot. 1988, 61, 117–125. [Google Scholar] [CrossRef] [Scilit]
- Finch-Savage, W.E.; Bassel, G.W. Seed vigour and crop establishment: Extending performance beyond adaptation. J. Exp. Bot. 2016, 67, 567–591. [Google Scholar] [CrossRef] [Scilit]
- Taiz, L.; Zeiger, E.; Møller, I.M.; Murphy, A. Plant Physiology and Development, 6th ed.; Sinauer Associates: Sunderland, MA, USA, 2015. [Google Scholar]
- Munns, R.; Tester, M. Mechanisms of salinity tolerance. Annu. Rev. Plant Biol. 2008, 59, 651–681. [Google Scholar] [CrossRef] [Scilit]
- Epstein, E.; Bloom, A.J. Mineral Nutrition of Plants: Principles and Perspectives, 2nd ed.; Sinauer Associates: Sunderland, MA, USA, 2005. [Google Scholar]
- Marschner, P. Marschner’s Mineral Nutrition of Higher Plants, 3rd ed.; Academic Press: London, UK, 2012. [Google Scholar]
- Murashige, T.; Skoog, F. A revised medium for rapid growth and bio assays with tobacco tissue cultures. Physiol. Plant. 1962, 15, 473–497. [Google Scholar] [CrossRef] [Scilit]
- George, E.F.; Hall, M.A.; De Klerk, G.-J. Plant Propagation by Tissue Culture, 3rd ed.; Springer: Dordrecht, The Netherlands, 2008. [Google Scholar]
- Bhattacharya, P.; Dey, S.; Bhattacharyya, B.C. Use of low-cost gelling agents and support matrices for industrial scale plant tissue culture. Plant Cell Tissue Organ Cult. 1994, 37, 15–23. [Google Scholar] [CrossRef] [Scilit]
- Cassells, A.C. Contamination and its impact in plant tissue culture. Methods Mol. Biol. 2012, 877, 57–80. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Leifert, C.; Cassells, A.C. Microbial hazards in plant tissue and cell cultures. In Vitro Cell. Dev. Biol.—Plant 2001, 37, 133–138. [Google Scholar] [CrossRef] [Scilit]
- Rezaei, H.; Mirzaie-asl, A.; Abdollahi, M.R.; Tohidfar, M. Comparative analysis of different artificial neural networks for predicting and optimizing in vitro seed germination and sterilization of petunia. PLoS ONE 2023, 18, e0285657. [Google Scholar] [CrossRef] [Scilit]
- Montgomery, D.C. Design and Analysis of Experiments, 8th ed.; John Wiley & Sons: Hoboken, NJ, USA, 2012. [Google Scholar]
- Tukey, J.W. Comparing individual means in the analysis of variance. Biometrics 1949, 5, 99–114. [Google Scholar] [CrossRef] [Scilit]
- Kruskal, W.H.; Wallis, W.A. Use of ranks in one-criterion variance analysis. J. Am. Stat. Assoc. 1952, 47, 583–621. [Google Scholar] [CrossRef]
- Wilcoxon, F. Individual comparisons by ranking methods. Biom. Bull. 1945, 1, 80–83. [Google Scholar] [CrossRef] [Scilit]
- Benjamini, Y.; Hochberg, Y. Controlling the false discovery rate: A practical and powerful approach to multiple testing. J. R. Stat. Soc. Ser. B 1995, 57, 289–300. [Google Scholar] [CrossRef] [Scilit]
- Jolliffe, I.T. Principal Component Analysis, 2nd ed.; Springer: New York, NY, USA, 2002. [Google Scholar] [CrossRef] [Scilit]
- Abdi, H.; Williams, L.J. Principal component analysis. WIREs Comput. Stat. 2010, 2, 433–459. [Google Scholar] [CrossRef] [Scilit]
- Husson, F.; Lê, S.; Pagès, J. Exploratory Multivariate Analysis by Example Using R, 2nd ed.; Chapman and Hall/CRC: Boca Raton, FL, USA, 2017. [Google Scholar] [CrossRef] [Scilit]
- Ward, J.H. Hierarchical grouping to optimize an objective function. J. Am. Stat. Assoc. 1963, 58, 236–244. [Google Scholar] [CrossRef]
- Kanjevac, M.; Jakovljević, D.; Todorović, M.; Stanković, M.; Ćurčić, S.; Bojović, B. Improvement of germination and early growth of radish (Raphanus sativus L.) through modulation of seed metabolic processes. Plants 2022, 11, 757. [Google Scholar] [CrossRef] [Scilit]
- International Seed Testing Association (ISTA). International Rules for Seed Testing 2024: Chapter 2: Sampling; ISTA: Bassersdorf, Switzerland, 2024. [Google Scholar]
- Lê, S.; Josse, J.; Husson, F. FactoMineR: An R package for multivariate analysis. J. Stat. Softw. 2008, 25, 1–18. [Google Scholar] [CrossRef] [Scilit]
- Kassambara, A.; Mundt, F. factoextra: Extract and Visualize the Results of Multivariate Data Analyses; R Package Version 1.0.7; Comprehensive R archive Network (CRAN): Vienna, Austria, 2020; Available online: https://CRAN.R-project.org/package=factoextra (accessed on 28 February 2026).
- R Core Team. R: A Language and Environment for Statistical Computing; R Foundation for Statistical Computing: Vienna, Austria, 2022. [Google Scholar]
- Bradford, K.J. Applications of hydrothermal time to quantifying and modeling seed germination and dormancy. Weed Sci. 2002, 50, 248–260. [Google Scholar] [CrossRef] [Scilit]
- Bradford, K.J. A water relations analysis of seed germination rates. Plant Physiol. 1990, 94, 840–849. [Google Scholar] [CrossRef] [Scilit]
- García-Huidobro, J.; Monteith, J.L.; Squire, G.R. Time, temperature and germination of pearl millet (Pennisetum typhoides S. & H.): I. CONSTANT TEMPERATURE. J. Exp. Bot. 1982, 33, 288–296. [Google Scholar] [CrossRef] [Scilit]
- Gummerson, R.J. The effect of constant temperatures and osmotic potentials on the germination of sugar beet. J. Exp. Bot. 1986, 37, 729–741. [Google Scholar] [CrossRef] [Scilit]
- Alvarado, V.; Bradford, K.J. A hydrothermal time model explains the cardinal temperatures for seed germination. Plant Cell Environ. 2002, 25, 1061–1069. [Google Scholar] [CrossRef] [Scilit]
- Watt, M.S.; Bloomberg, M.; Finch-Savage, W.E. Development of a hydrothermal time model that accurately characterises how thermoinhibition regulates germination. Ecol. Model. 2010, 221, 1267–1272. [Google Scholar] [CrossRef] [Scilit]
- Mesgaran, M.B.; Mashhadi, H.R.; Alizadeh, H.; Hunt, J.; Young, K.R.; Cousens, R.D. Importance of distribution function selection for hydrothermal time models of seed germination. Weed Res. 2013, 53, 89–101. [Google Scholar] [CrossRef] [Scilit]
- Onofri, A.; Benincasa, P.; Mesgaran, M.B.; Ritz, C. Hydrothermal-time-to-event models for seed germination. Eur. J. Agron. 2018, 101, 129–139. [Google Scholar] [CrossRef] [Scilit]
- Czabator, F.J. Germination value: An index combining speed and completeness of pine seed germination. For. Sci. 1962, 8, 386–396. [Google Scholar] [CrossRef] [Scilit]
- Djavanshir, K.; Pourbeik, H. Germination value—A new formula. Silvae Genet. 1976, 25, 79–83. [Google Scholar]
- Lv, Y.Y.; Wang, Y.R.; Powell, A.A. Frequent individual counts of radicle emergence and mean just germination time predict seed vigour of Avena sativa and Elymus nutans. Seed Sci. Technol. 2016, 44, 189–198. [Google Scholar] [CrossRef] [Scilit]
- Bro, R.; Smilde, A. Principal component análisis. Anal. Methods 2014, 6, 2812–2831. [Google Scholar] [CrossRef] [Scilit]
- Carrera-Castaño, G.; Calleja-Cabrera, J.; Pernas, M.; Gómez, L. An Updated Overview on the Regulation of Seed Germination. Plants 2020, 9, 703. [Google Scholar] [CrossRef] [Scilit]
- Labouriau, L.G. A Germinação de Sementes; Secretaria Geral da OEA: Brasilia, Brazil, 1983. [Google Scholar]
- De Sousa Basílio, A.M.; Da Silva, M.A.M.; Santana, C.C. Potencial osmótico e concentração de cloreto de sódio na germinação de sementes de rabanete. Rev. Ciênc. Agrár. 2018, 41, 638–648. [Google Scholar]
- Viciedo, D.O.; Prado, R.M.; Martinez, H.E.P.; Gratão, P.L. Silicon supplementation alleviates ammonium toxicity in radish plants. J. Sci. Food Agric. 2020, 100, 3525–3531. [Google Scholar] [CrossRef] [Scilit]
- Almansouri, M.; Kinet, J.M.; Lutts, S. Effect of salt and osmotic stresses on germination in durum wheat seeds. Plant Soil. 2001, 231, 243–254. [Google Scholar] [CrossRef] [Scilit]
- Radouani, A.; Lauer, F.I.; Abdelmajid, K. Effect of NPK media concentrations on in vitro potato tuberization of cultivars Nicola and Russet Burbank. Am. J. Potato Res. 2015, 92, 146–155. [Google Scholar] [CrossRef] [Scilit]
- Fiorani, F.; Schurr, U. Future scenarios for plant phenotyping. Annu. Rev. Plant Biol. 2013, 64, 267–291. [Google Scholar] [CrossRef] [Scilit]
- Schindelin, J.; Arganda-Carreras, I.; Frise, E.; Kaynig, V.; Longair, M.; Pietzsch, T.; Preibisch, S.; Rueden, C.; Saalfeld, S.; Schmid, B.; et al. Fiji: An open-source platform for biological-image analysis. Nat. Methods 2012, 9, 676–682. [Google Scholar] [CrossRef] [Scilit]
- Hmissi, M.; Chaieb, M.; Krouma, A. Differences in the Physiological Indicators of Seed Germination and Seedling Establishment of Durum Wheat (Triticum durum Desf.) Cultivars Subjected to Salinity Stress. Agronomy 2023, 13, 1718. [Google Scholar] [CrossRef] [Scilit]
- Toscano, S.; Romano, D.; Tribulato, A.; Rizzo, V. Annual garden rocket and radish as microgreens: Seed germination response to thermal and salt stress. Agronomy 2025, 15, 361. [Google Scholar] [CrossRef] [Scilit]
- Benjamini, Y.; Yekutieli, D. The control of the false discovery rate in multiple testing under dependency. Ann. Stat. 2001, 29, 1165–1188. [Google Scholar] [CrossRef] [Scilit]
- Holm, S. A simple sequentially rejective multiple test procedure. Scand. J. Stat. 1979, 6, 65–70. [Google Scholar]
- Gamborg, O.L.; Miller, R.A.; Ojima, K. Nutrient requirements of suspension cultures of soybean root cells. Exp. Cell Res. 1968, 50, 151–158. [Google Scholar] [CrossRef] [Scilit]
- Lloyd, G.; McCown, B. Commercially-feasible micropropagation of mountain laurel, Kalmia latifolia, by use of shoot-tip culture. Proc. Int. Plant Prop. Soc. 1980, 30, 421–427. [Google Scholar]
- Paparella, S.; Araújo, S.S.; Rossi, G.; Wijayasinghe, M.; Carbonera, D.; Balestrazzi, A. Seed priming: State of the art and new perspectives. Plant Cell Rep. 2015, 34, 1281–1293. [Google Scholar] [CrossRef] [Scilit]
- Ashraf, M.; Foolad, M.R. Pre-sowing seed treatment—A shotgun approach to improve germination and seedling growth under salt and drought stress. Adv. Agron. 2005, 88, 223–271. [Google Scholar]
- Finch-Savage, W.E.; Leubner-Metzger, G. Seed dormancy and the control of germination. New Phytol. 2006, 171, 501–523. [Google Scholar] [CrossRef] [Scilit]
- Alboresi, A.; Gestin, C.; Leydecker, M.-T.; Bedu, M.; Meyer, C.; Truong, H.-N. Nitrate, a signal relieving seed dormancy in Arabidopsis. Plant Cell Environ. 2005, 28, 500–512. [Google Scholar] [CrossRef] [Scilit]
- Duermeyer, L.; Khodapanahi, E.; Yan, D.; Krapp, A.; Rothstein, S.J.; Nambara, E. Regulation of seed dormancy and germination by nitrate. Seed Sci. Res. 2018, 28, 150–157. [Google Scholar] [CrossRef] [Scilit]
- Bethke, P.C.; Gubler, F.; Jacobsen, J.V.; Jones, R.L. Dormancy of Arabidopsis seeds and barley grains can be broken by nitric oxide. Plant Physiol. 2006, 140, 170–179. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, H.; Wang, R.; Wang, X.; Zhao, C.; Shen, H.; Yang, L. Nitric oxide regulates seed germination: Integrating hormone signaling and reactive oxygen species. Int. J. Mol. Sci. 2023, 24, 9052. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- López-Bucio, J.; Cruz-Ramírez, A.; Herrera-Estrella, L. The role of nutrient availability in regulating root architecture. Curr. Opin. Plant Biol. 2003, 6, 280–287. [Google Scholar] [CrossRef] [Scilit]
- Gruber, B.D.; Giehl, R.F.H.; Friedel, S.; von Wirén, N. Plasticity of the Arabidopsis root system under nutrient deficiencies. Plant Physiol. 2013, 163, 161–179. [Google Scholar] [CrossRef] [Scilit]
- Lynch, J.P. Root phenes for enhanced soil exploration and phosphorus acquisition: Tools for future crops. Plant Physiol. 2011, 156, 1041–1049. [Google Scholar] [CrossRef] [Scilit]
- Choi, I.; Cho, H.; Brandizzi, F.; Rouached, H. Phosphorus deficiency and root growth: The role of TOR signaling in adaptive responses. J. Exp. Bot. 2026, 77, 1375–1383. [Google Scholar] [CrossRef] [Scilit]
- Legendre, P.; Legendre, L. Numerical Ecology, 3rd English ed.; Elsevier: Amsterdam, The Netherlands, 2012. [Google Scholar]
- Kaufman, L.; Rousseeuw, P.J. Finding Groups in Data: An Introduction to Cluster Analysis; Wiley: New York, NY, USA, 1990. [Google Scholar]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.