


Abstract
The Muški bunar old-growth forest on Mount Psunj represents one of the rare preserved mixed ecosystems of sessile oak (Quercus petraea (Matt.) Liebl.) and European beech (Fagus sylvatica L.) in Southeastern Europe, providing an important reference for understanding natural forest dynamics. This study aimed to analyse stand structure, age distribution, growth dynamics, and disturbance regime based on repeated field surveys conducted in 1979 and 2021. The results revealed pronounced structural heterogeneity and clear interspecific differences. European beech dominates smaller- and medium-diameter classes, as well as a wider range of age classes, whereas sessile oak is primarily present in older and larger diameter classes. A very high growing stock (1155.81 m3 ha−1) indicates exceptional stand productivity, with maximum cambial ages of 295 years for oak and 253 years for beech. Basal area increment analysis showed that both species maintain substantial growth at advanced ages. However, recent decades show divergence, with increasing growth in beech and stagnation or decline in oak. Importantly, growth releases in sessile oak were not accompanied by successful regeneration, indicating a decoupling between growth response and recruitment. Stand dynamics are mainly driven by low-intensity disturbances. These findings highlight the importance of old-growth forests as reference systems and improve understanding of species-specific responses to disturbance.
1. Introduction
Understanding the structure and dynamics of old-growth forest ecosystems is increasingly important in the context of global change and the development of resilient forest systems. Primary and old-growth forests serve as key reference ecosystems for understanding long-term forest functioning and development in Europe [1,2]. Despite strong anthropogenic pressures that have reduced their extent, the remaining preserved fragments provide valuable insights into natural processes shaping forest structure, stability, and resilience [2].
Old-growth forests are characterized by high structural heterogeneity, including a wide range of tree sizes, multilayered canopy structure, and substantial amounts of deadwood [3]. This heterogeneity arises from long-term interactions among natural disturbances, species-specific ecological traits, and environmental conditions [4,5]. Canopy gap dynamics, particularly those driven by wind disturbances, represent a key mechanism shaping forest structure and spatial variability [6,7], although their relative importance in stand development remains debated [5,8]. Studies from the Dinaric and Carpathian regions demonstrate that disturbance, competition, and mortality jointly drive the development of structurally complex stands [9,10].
In mixed forests of European beech (Fagus sylvatica L.) and sessile oak (Quercus petraea (Matt.) Liebl.), stand structure is strongly influenced by contrasting species-specific ecological strategies. European beech is one of the most widespread tree species in temperate Europe and forms both monospecific stands in montane zones and mixed stands with silver fir (Abies alba Mill.) in the Dinaric region, where species coexistence mechanisms are well understood and have supported the development of close-to-nature forest management concepts [9,11,12,13]. In contrast, such models remain less developed for mixed beech–oak stands under more continental and drier conditions. Previous research indicates that beech–oak old-growth forests exhibit pronounced structural complexity and specific regeneration patterns driven primarily by differences in species light requirements. These stands are characterized by heterogeneous diameter and age structures, high variability in tree dimensions, and marked spatial heterogeneity associated with canopy gap dynamics [5,8,14]. Beech regenerates continuously in small canopy gaps, whereas oak regeneration is limited to larger and more intense disturbances, resulting in its dominance in older age classes [8]. Consequently, gap size and disturbance intensity play a key role in regulating species composition and long-term stand dynamics. However, long-term structural and growth dynamics of mixed beech–oak old-growth forests under continental conditions in Southeastern Europe remain poorly quantified, particularly regarding the interaction between stand structure, tree age, and disturbance regimes. Furthermore, the rarity of preserved old-growth stands of this forest type significantly limits opportunities for systematic research [2,8]. In this context, long-term inventories of old-growth forest structure provide a unique opportunity to analyse forest development under near-natural conditions, including growth, mortality, and regeneration dynamics.
This study aims to quantify long-term changes in stand structure of a sessile oak–European beech old-growth forest based on repeated inventories (1979–2021), and to analyse its age structure, growth dynamics, and disturbance regime.
The following hypotheses were tested:
H1.
Stand structure changes significantly over time, reflected in increases in tree dimensions, basal area, and growing stock as a result of natural development.
H2.
The age structure reflects a multi-cohort dynamic, with European beech represented across a wider range of age classes and showing continuous regeneration, whereas sessile oak is predominantly concentrated in older age classes.
2. Materials and Methods
2.1. Study Area
The study was conducted in the Muški bunar old-growth forest reserve (45.3490975° N, 17.2899176° E), located in the southwestern part of the Psunj mountain massif (western Croatia), at elevations ranging from 680 to 807 m a.s.l. The reserve represents a remnant of formerly more widespread mixed forests of oak and beech and covers an area of 46 ha. The forest consists of two spatially and ecologically distinct units. The upper northeastern part (approximately 24 ha), characterized by a gently levelled plateau, is dominated by a pure beech stand, classified as the association Cephalanthero longifoliae–Fagetum ass. nov. [15]. In contrast, the lower southwestern part (approximately 22 ha), characterized by convex hilltops and steep slopes, is occupied by a mixed beech–sessile oak stand, which can be interpreted as a subassociation with sessile oak [16]. According to historical records, the area has not been subject to direct anthropogenic influence. It was excluded from regular forest management in 1929 and designated as a special forest vegetation reserve in 1963.
2.2. Climatic and Site Characteristics
The reserve area is characterized by a humid temperate climate with a slight sub-Mediterranean influence. The mean annual temperature is approximately 7 °C, and the total annual precipitation is about 1125 mm. The geological substrate consists of acidic silicate rocks (schists), while soils are predominantly shallow and skeletal on steep slopes, and deeper dystric brown soils and Luvisols on gentler terrain. Mixed beech–oak stands develop on drier and shallower soils, whereas pure beech stands occur on deeper and more mesic microsites.
2.3. Sampling and Field Measurements
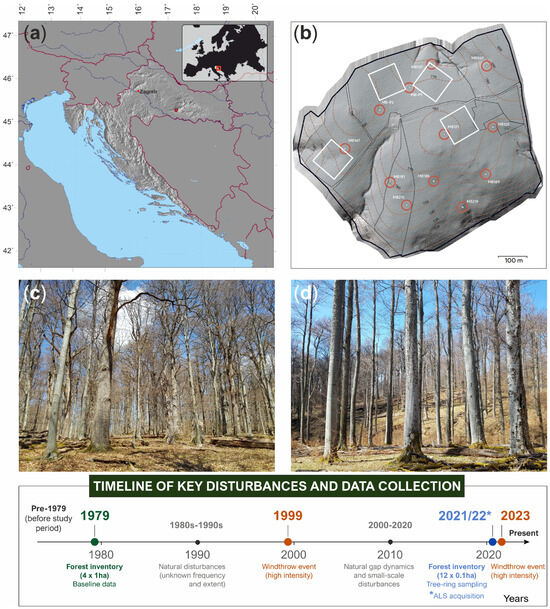
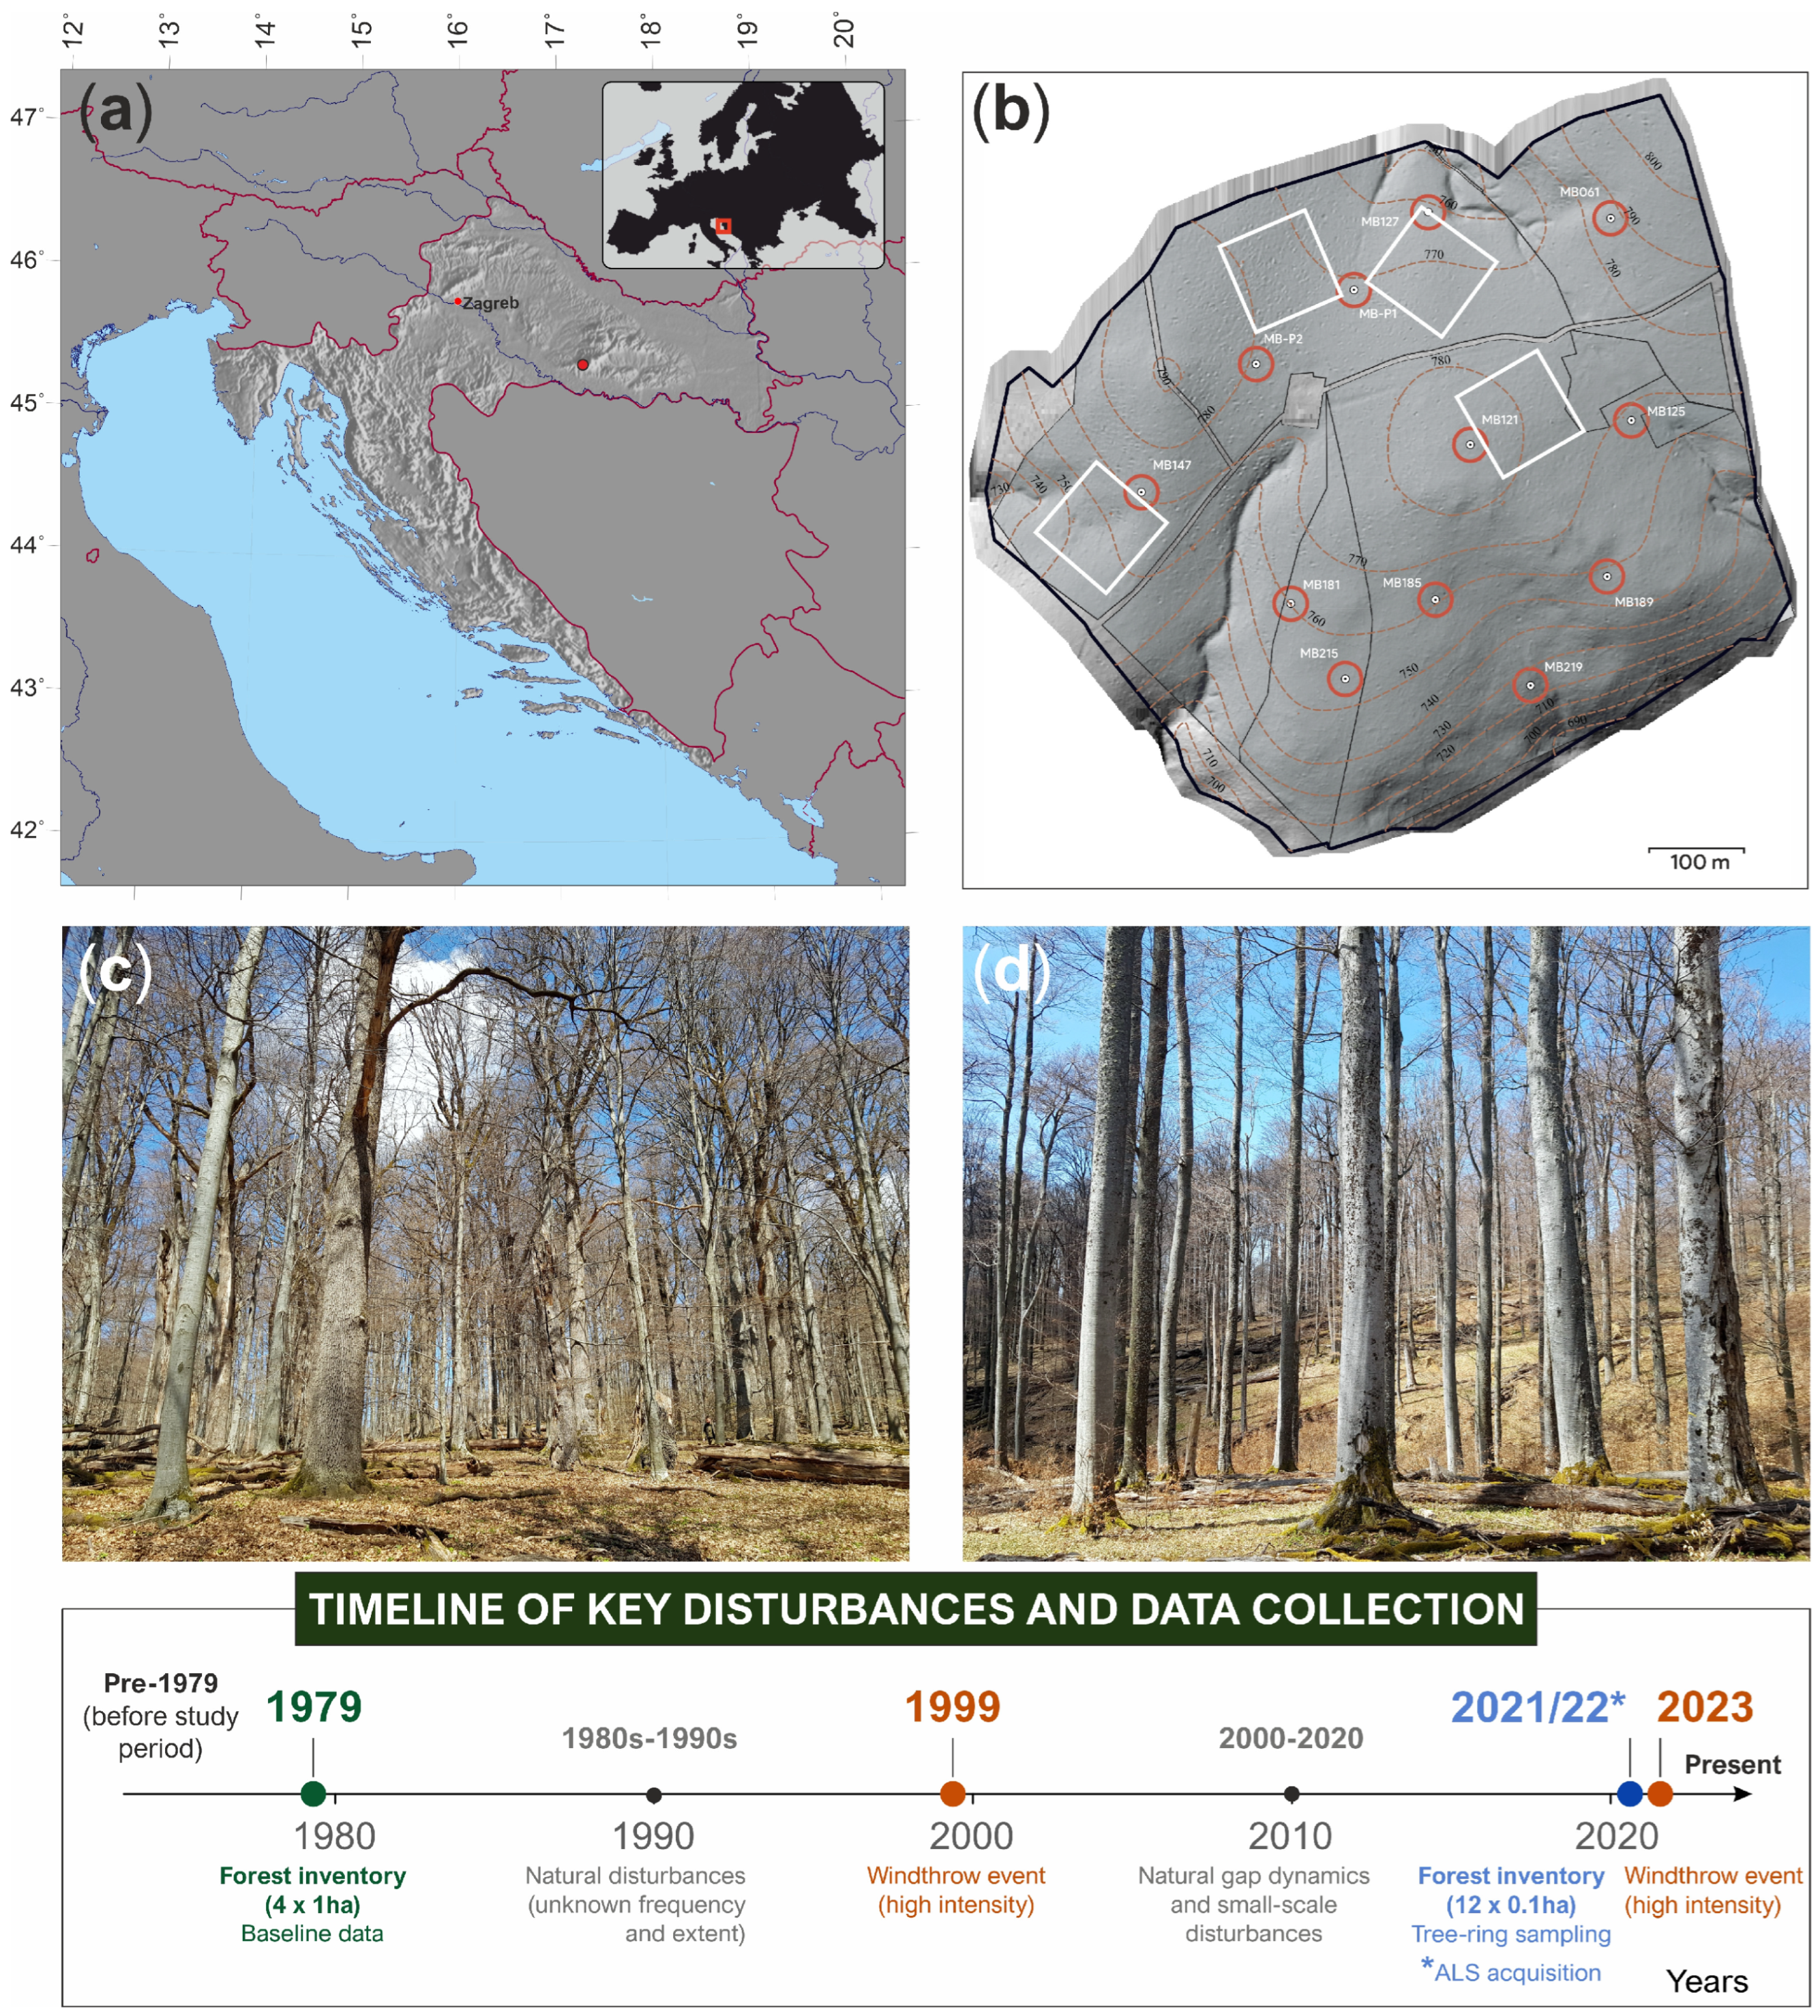
Initial research in the reserve was conducted in 1979 within the framework of the Man and the Biosphere (MAB) project [16]. During the 1990s, the area was located within occupied territory and classified as a mine-suspected area, which restricted access until complete demining in 2017 and significantly limited research activities. Field investigations resumed in 2021, when twelve circular sample plots (1000 m2; radius 17.81 m) were established, covering a total area of 1.2 ha (approximately 2.6% of the reserve). The plots were systematically distributed to ensure representative coverage of the study area (Figure 1b). Within each plot, diameter at breast height (DBH, cm) and tree height (m) were measured for all trees with DBH ≥ 10 cm. Standing dead trees and downed deadwood with diameters > 10 cm were also recorded and classified into five standard decay classes. Deadwood was not assessed during the 1979 inventory; therefore, no comparative data are available for this component. For dendroecological analyses, two increment cores per tree were extracted from all sampled trees using a Haglöf Pressler increment borer (Haglöf Sweden AB, Långsele, Sweden; 4.9 mm diameter) at 1 m above ground level. In total, 230 trees were sampled, including 184 beech and 46 oak. The samples were stored in plastic straws in the field and processed in the laboratory following standard dendrochronological procedures [17]. Core samples were prepared using a Core-Microtome WSL (WSL, Birmensdorf, Switzerland) to enable precise measurement of tree-ring widths.
Figure 1.
Study area and sampling design of the Muški bunar old-growth forest. (a) Geographic location of the study area in Croatia; (b) spatial distribution of sample plots established in 2021 (red circles) and location of the 1979 inventory plots (white squares; 1 ha each); (c) mixed sessile oak–European beech stand; (d) beech-dominated stand. The lower panel illustrates the timeline of key disturbance events and data collection, including the 1979 and 2021 inventories, dendroecological sampling, ALS data acquisition, and major windthrow events in 1999 and 2023.
2.4. Tree-Ring Width Measurement
Tree-ring widths (TRW) were measured using CooRecorder 9.6 software (Cybis Elektronik & Data AB, Saltsjöbaden, Sweden; https://www.cybis.se) on digital images acquired with the ATRICS (Advanced Tree Ring Image Capturing System) [18]. The system was equipped with a motorized measurement stage Isel MS200HT, (isel Germany AG, Eichenzell, Germany), a stereomicroscope (Zeiss Stemi 305, Zeiss, Munich, Germany), and a digital camera (Infinity Lumenera 1, Teledyne Vision Solutions, Ottawa, ON, Canada). For each sample, tree age was estimated using the “distance to pith” tool implemented in CooRecorder. Samples with estimated missing segments corresponding to ≥10 rings were excluded from age-related analyses. As increment cores were extracted at 1.3 m above ground level, the estimated age represents tree age at sampling height rather than total biological age. To minimize potential bias associated with age estimation, trees were grouped into 10-year age classes. Cross-dating and synchronization of tree-ring series were performed using visual inspection and statistical analysis in TSAP-Win™ (version 4.81) (Rinntech, Heidelberg, Germany, http://www.rinntech.de). Dating accuracy was assessed using Student’s t-values based on correlation coefficients [19] and the Gleichläufigkeit (GLK) coefficient [20]. Quality control of cross-dating was further verified using COFECHA (version 6.06P) [21]. Finally, successfully dated individual series were averaged at the tree level to obtain mean tree-ring width series (TRWt).
2.5. Data Analysis and Processing
Stand structural attributes, particularly tree volume, were calculated using Schumacher–Hall equations with locally calibrated coefficients for oak and beech. Calculations followed the methodology applied in the 1979 inventory [16]. Comparison of results between the two inventories required careful consideration of differences in sampling design. The 1979 inventory was conducted on four plots of 1 ha each, whereas the recent study was based on a larger number of smaller plots (12 plots of 1000 m2). Such differences can influence the estimation of stand structural attributes, particularly in heterogeneous old-growth forests, where plot size affects the probability of capturing large trees and extreme values. Larger plots have a higher probability of capturing such elements and better integrate spatial variability, whereas smaller plots may result in higher variance and potential underestimation of extreme values. However, the increased number of plots in the recent inventory partially compensates for this limitation through improved spatial coverage and representativeness, which is particularly important in structurally complex stands. Importantly, comparable measurement criteria and volume estimation models were applied in both inventories, ensuring methodological consistency and enabling interpretation of temporal changes. The results can therefore be considered a reliable basis for analysing long-term structural dynamics, while acknowledging the limitations associated with sampling design. This limitation should be considered when comparing structural attributes between inventories.
2.6. Growth Release Analysis
Growth release dynamics were analysed using tree-ring width series from all plots, excluding two plots located within the 1999 windthrow area, resulting in a total of 197 samples. For each tree, the percentage growth change (%GC) in radial increment was calculated following the method described in [22], based on comparisons of mean growth over consecutive 10-year periods. Percentage growth change (%GC) was calculated as %GC = ((M2 − M1)/M1) × 100, where M1 represents the mean growth of the preceding 10-year period (excluding the target year), and M2 represents the mean growth of the subsequent 10-year period (including the target year). Thresholds for moderate and major growth releases (≥25% and >50%) follow established criteria [22]. The proportion of trees exhibiting a growth release was analysed over time to assess disturbance dynamics. All analyses were conducted using the package TRADER [23] in R (version 4.4.0).
2.7. Basal Area Increment (BAI)
Long-term growth trends were analysed using time series of annual basal area increment (BAI). BAI was calculated using the bai.out function from the package dplR [24] in R (version 4.4.0), based on diameter at breast height (DBH) and tree-ring width (TRW) series. Individual BAI series were aggregated into species-specific chronologies to enable a comparative analysis of growth patterns between beech and oak. Basal area increment, expressed in mm2, represents the annual increase in the cross-sectional area of a tree stem and is therefore considered one of the most reliable indicators of long-term tree growth.
2.8. Canopy Gap Analysis
Canopy gap analysis was performed using a canopy height model (CHM) derived from airborne laser scanning (ALS) data acquired within the national project “Multi-sensor Airborne Survey of the Republic of Croatia for Disaster Risk Reduction” (KK.05.2.1.10.0001). The ALS data used to generate the canopy height model (CHM) were acquired in 2022. The CHM, with a spatial resolution of 1 m, was generated from the ALS point cloud by deriving a digital terrain model (DTM) and a digital surface model (DSM), from which canopy heights were calculated. Canopy gaps were identified using the package ForestGapR [25] in R (version 4.4.0), which enables automated detection and analysis of forest gaps based on CHM data. A canopy height threshold of 15 m was applied to delineate gaps. In CHM-based studies, threshold values for gap definition vary depending on ecological context and stand structure, typically ranging from a few metres up to approximately 20 m [26].
3. Results
3.1. Structural Characteristics of the Muški Bunar Old-Growth Forest
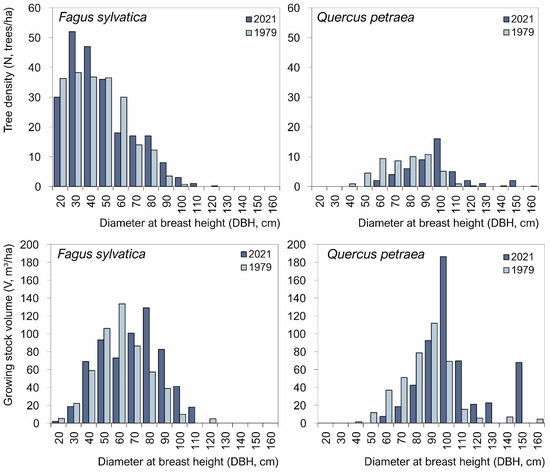
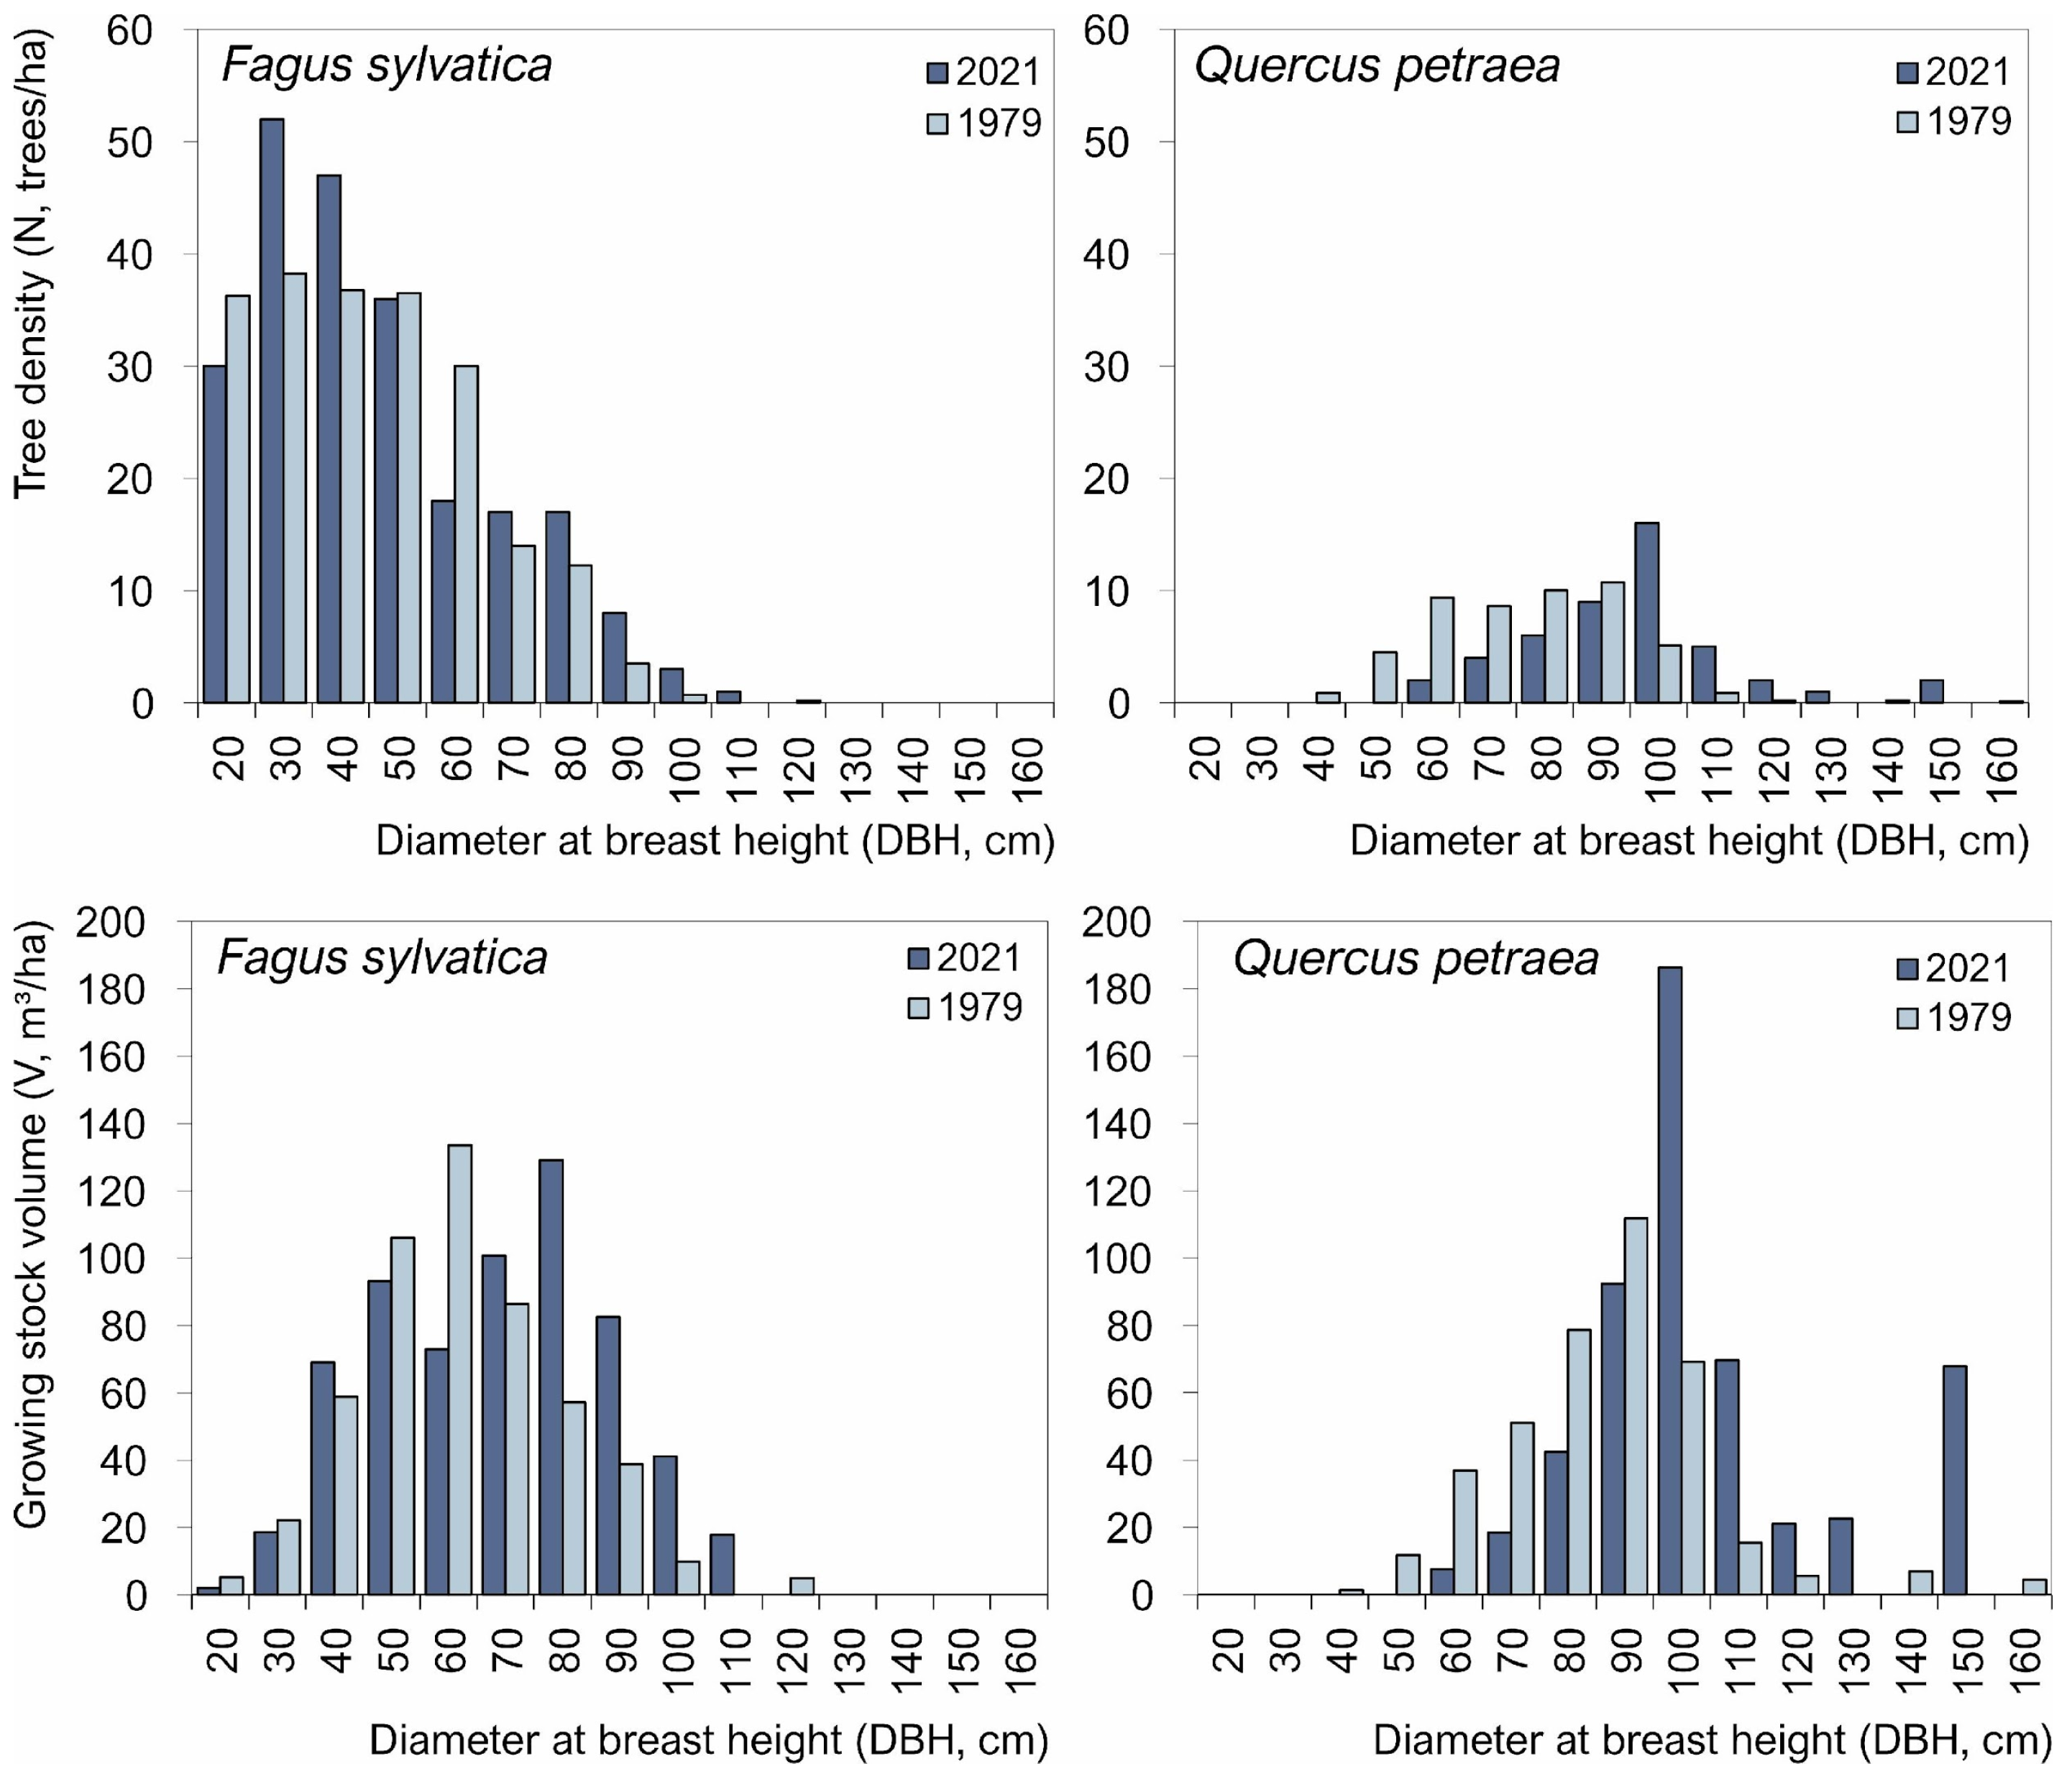
Comparison of stand structural characteristics between the 1979 and 2021 inventories indicates pronounced changes in stand structure. Over the 42-year period, total tree density slightly increased from 258 to 276 trees ha−1, while basal area increased from 51.66 to 66.84 m2 ha−1 and total volume from 911.44 to 1155.81 m3 ha−1, indicating substantial biomass accumulation. At the species level, beech increased its share in the stand, whereas sessile oak showed a slight decline in tree density but an increase in basal area and volume, reflecting the persistence of large individuals. Maximum tree dimensions confirm old-growth characteristics, with DBH reaching 106 cm for beech and 150 cm for oak, and tree heights up to 44 m and 40.2 m, respectively. For a given diameter, beech generally attained greater heights than oak. The average deadwood volume recorded in 2021 was 101.36 m3 ha−1, indicating a high level of structural complexity. Diameter distributions further highlight species-specific patterns. European beech was predominantly represented in smaller and medium diameter classes, whereas sessile oak was mainly concentrated in larger diameter classes, indicating ageing of the existing population (Figure 2).
Figure 2.
Distribution of stand density and growing stock volume across diameter classes (10 cm) by tree species for the entire reserve, comparing the 1979 and 2021 inventories.
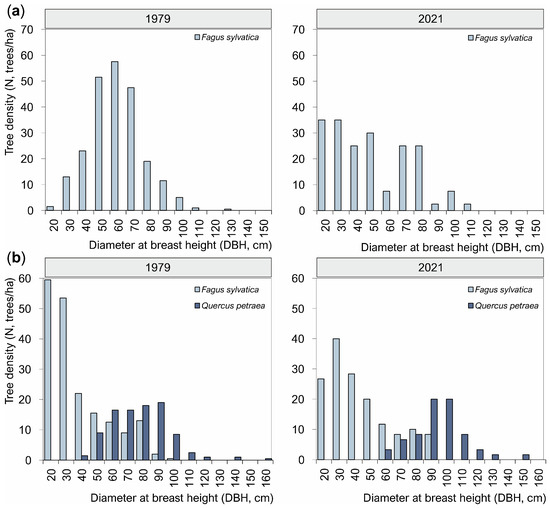
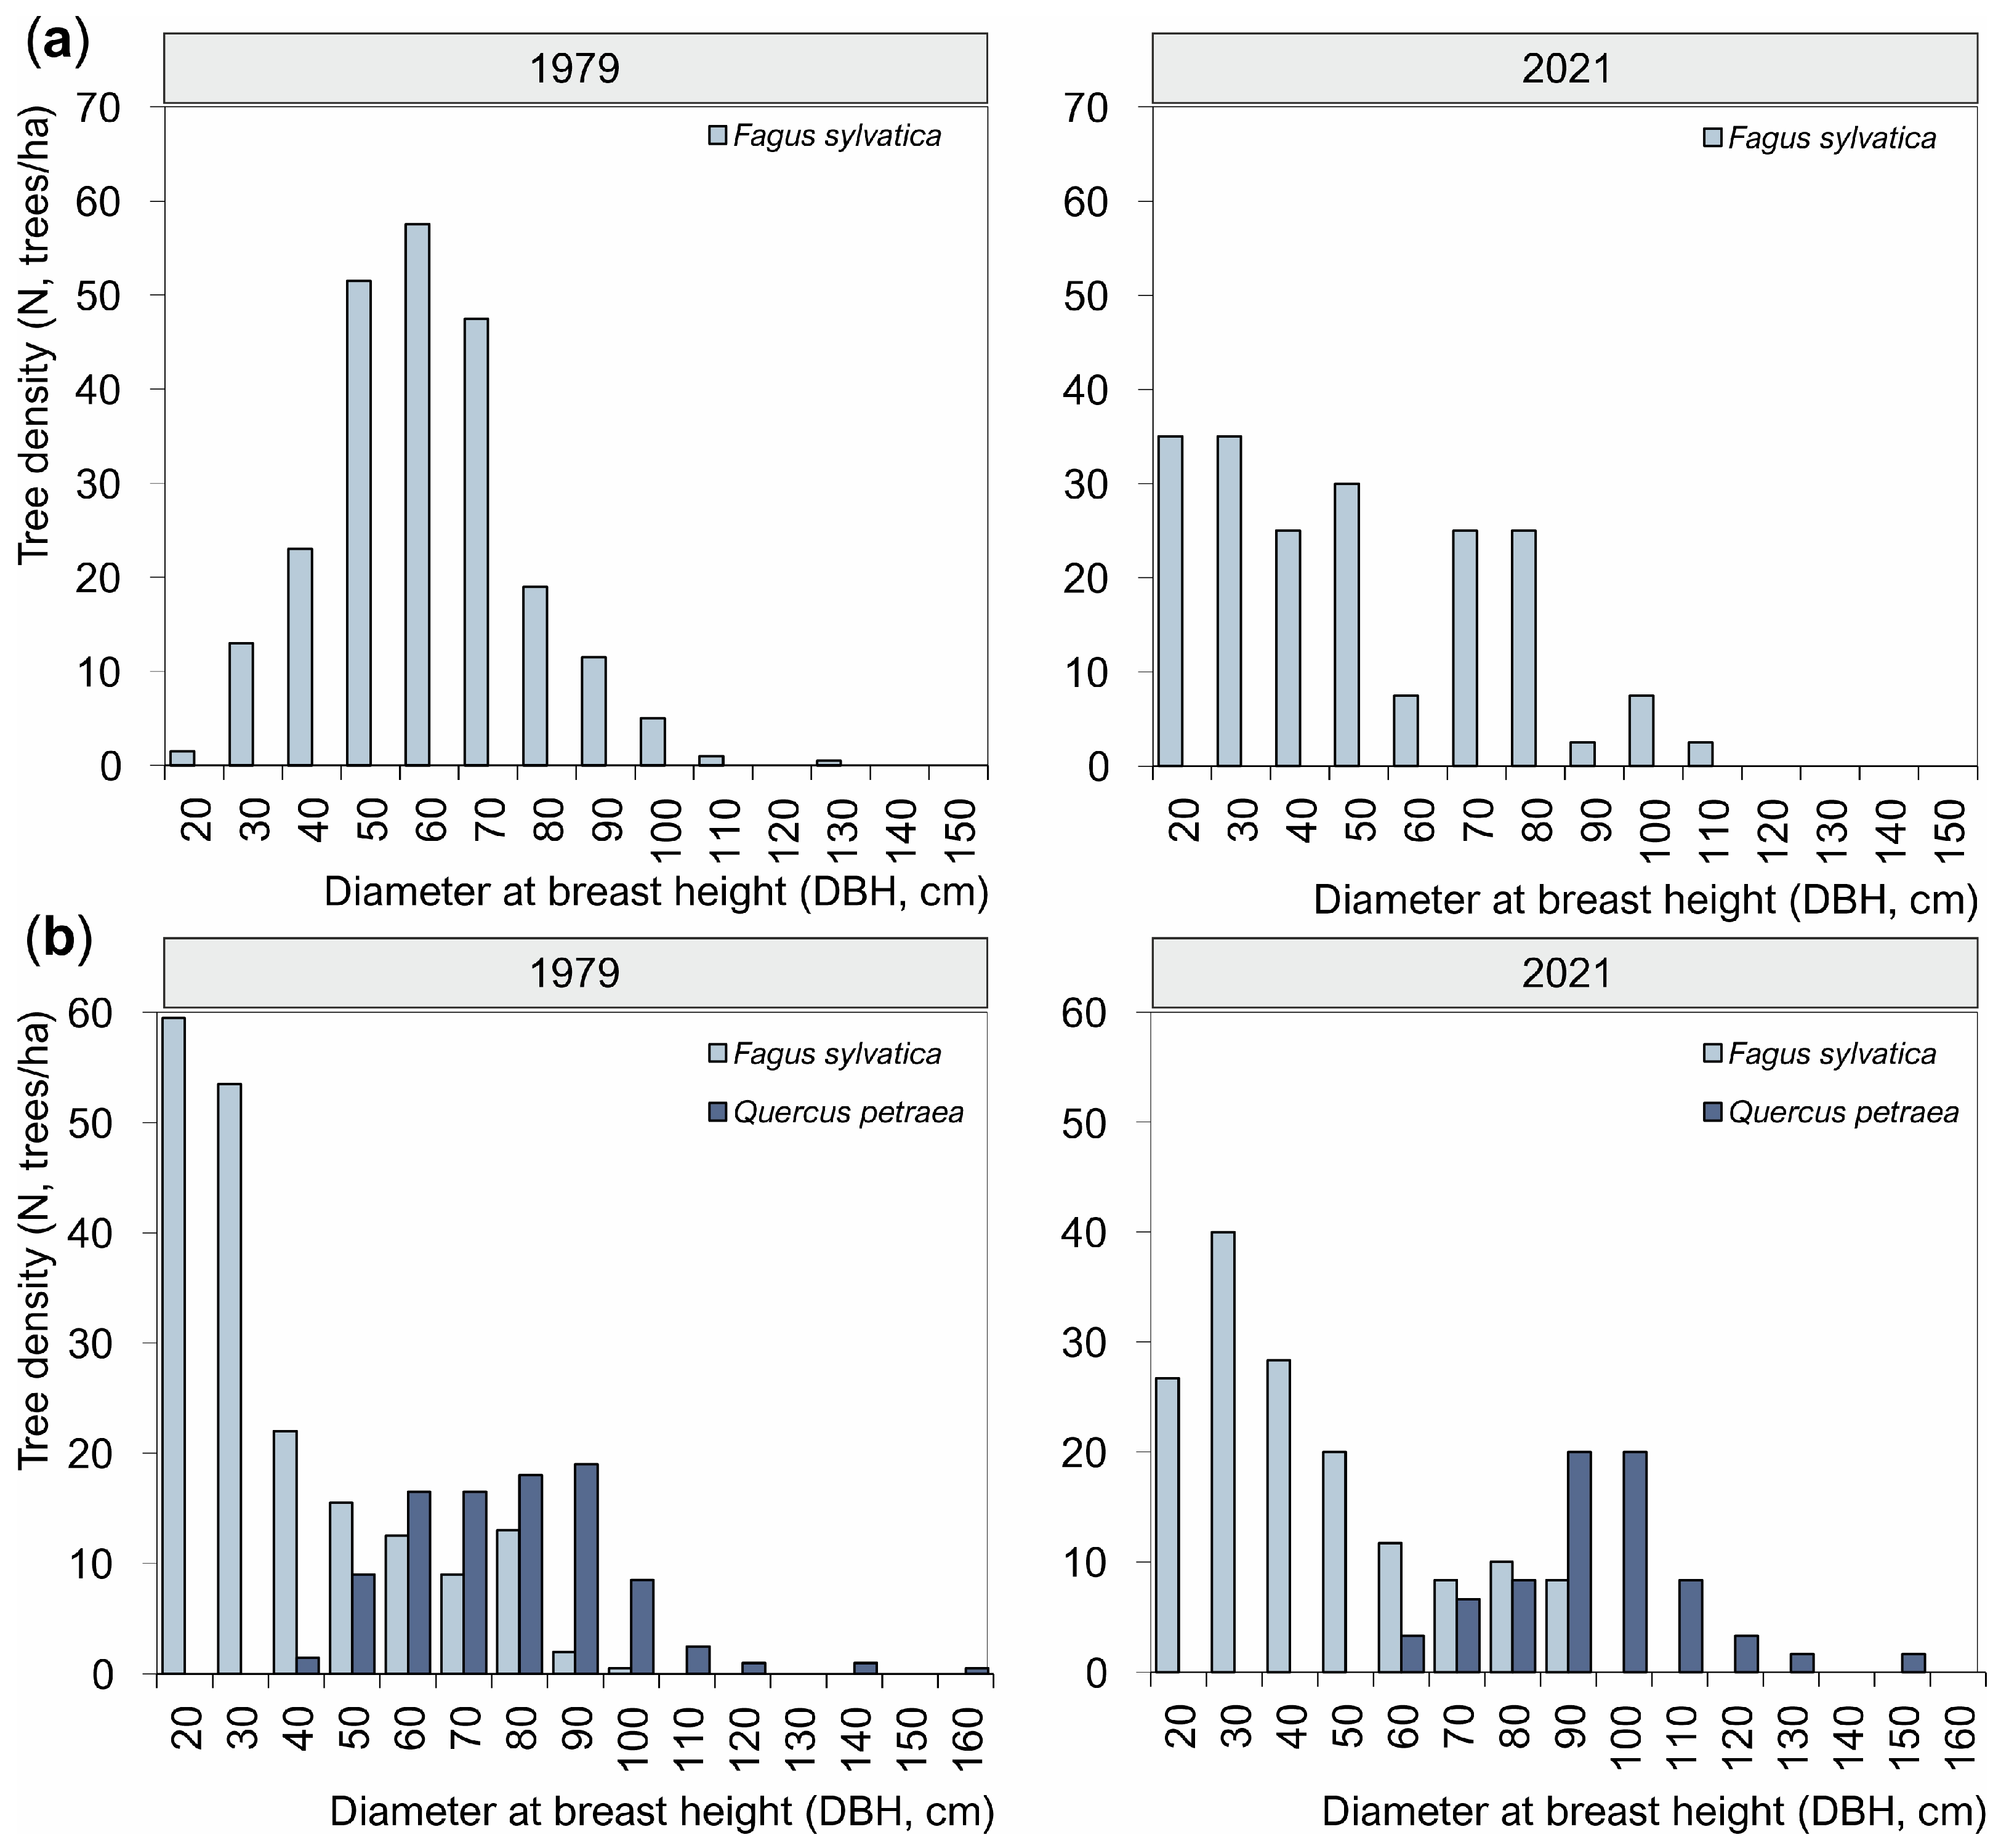
Structural changes differed between stand types. In pure beech stands, tree density decreased (from 231 to 203 trees ha−1), while basal area and stand volume increased moderately (from 43.45 to 46.00 m2 ha−1 and from 778.05 to 823.39 m3 ha−1, respectively). In contrast, changes in the mixed beech–oak stand were more pronounced, with a stronger decrease in tree density (from 282 to 227 trees ha−1) accompanied by a substantial increase in basal area (from 65.30 to 71.88 m2 ha−1) and volume (from 1035.55 to 1230.32 m3 ha−1). In 2021, beech dominated in terms of tree density (153 trees ha−1), whereas oak, although less abundant (73 trees ha−1), contributed most to total basal area and growing stock, reflecting differences in size structure between the two species. Diameter distributions further illustrate these patterns (Figure 3). In the pure beech stand, the distribution shifted from a unimodal to a more complex structure, indicating increased structural heterogeneity. In the mixed stand, distributions were irregular and bimodal, with beech concentrated in smaller diameter classes and sessile oak in medium and larger classes. Over time, a decline in beech trees in the smallest diameter classes was observed, indicating reduced recent recruitment into these classes.
Figure 3.
Tree density distribution across diameter classes by species in (a) pure beech stand and (b) mixed sessile oak–beech stand based on data from the 1979 and 2021 inventories.
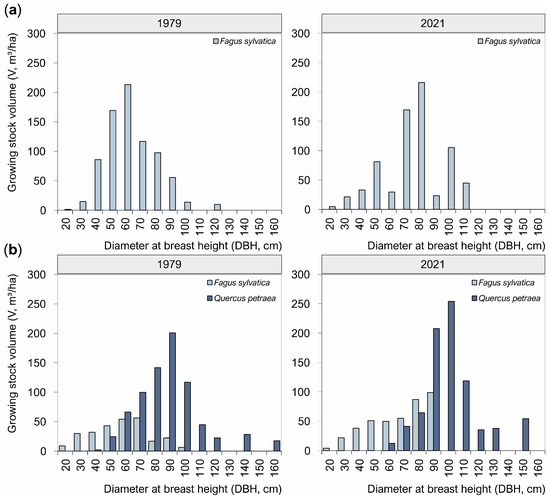
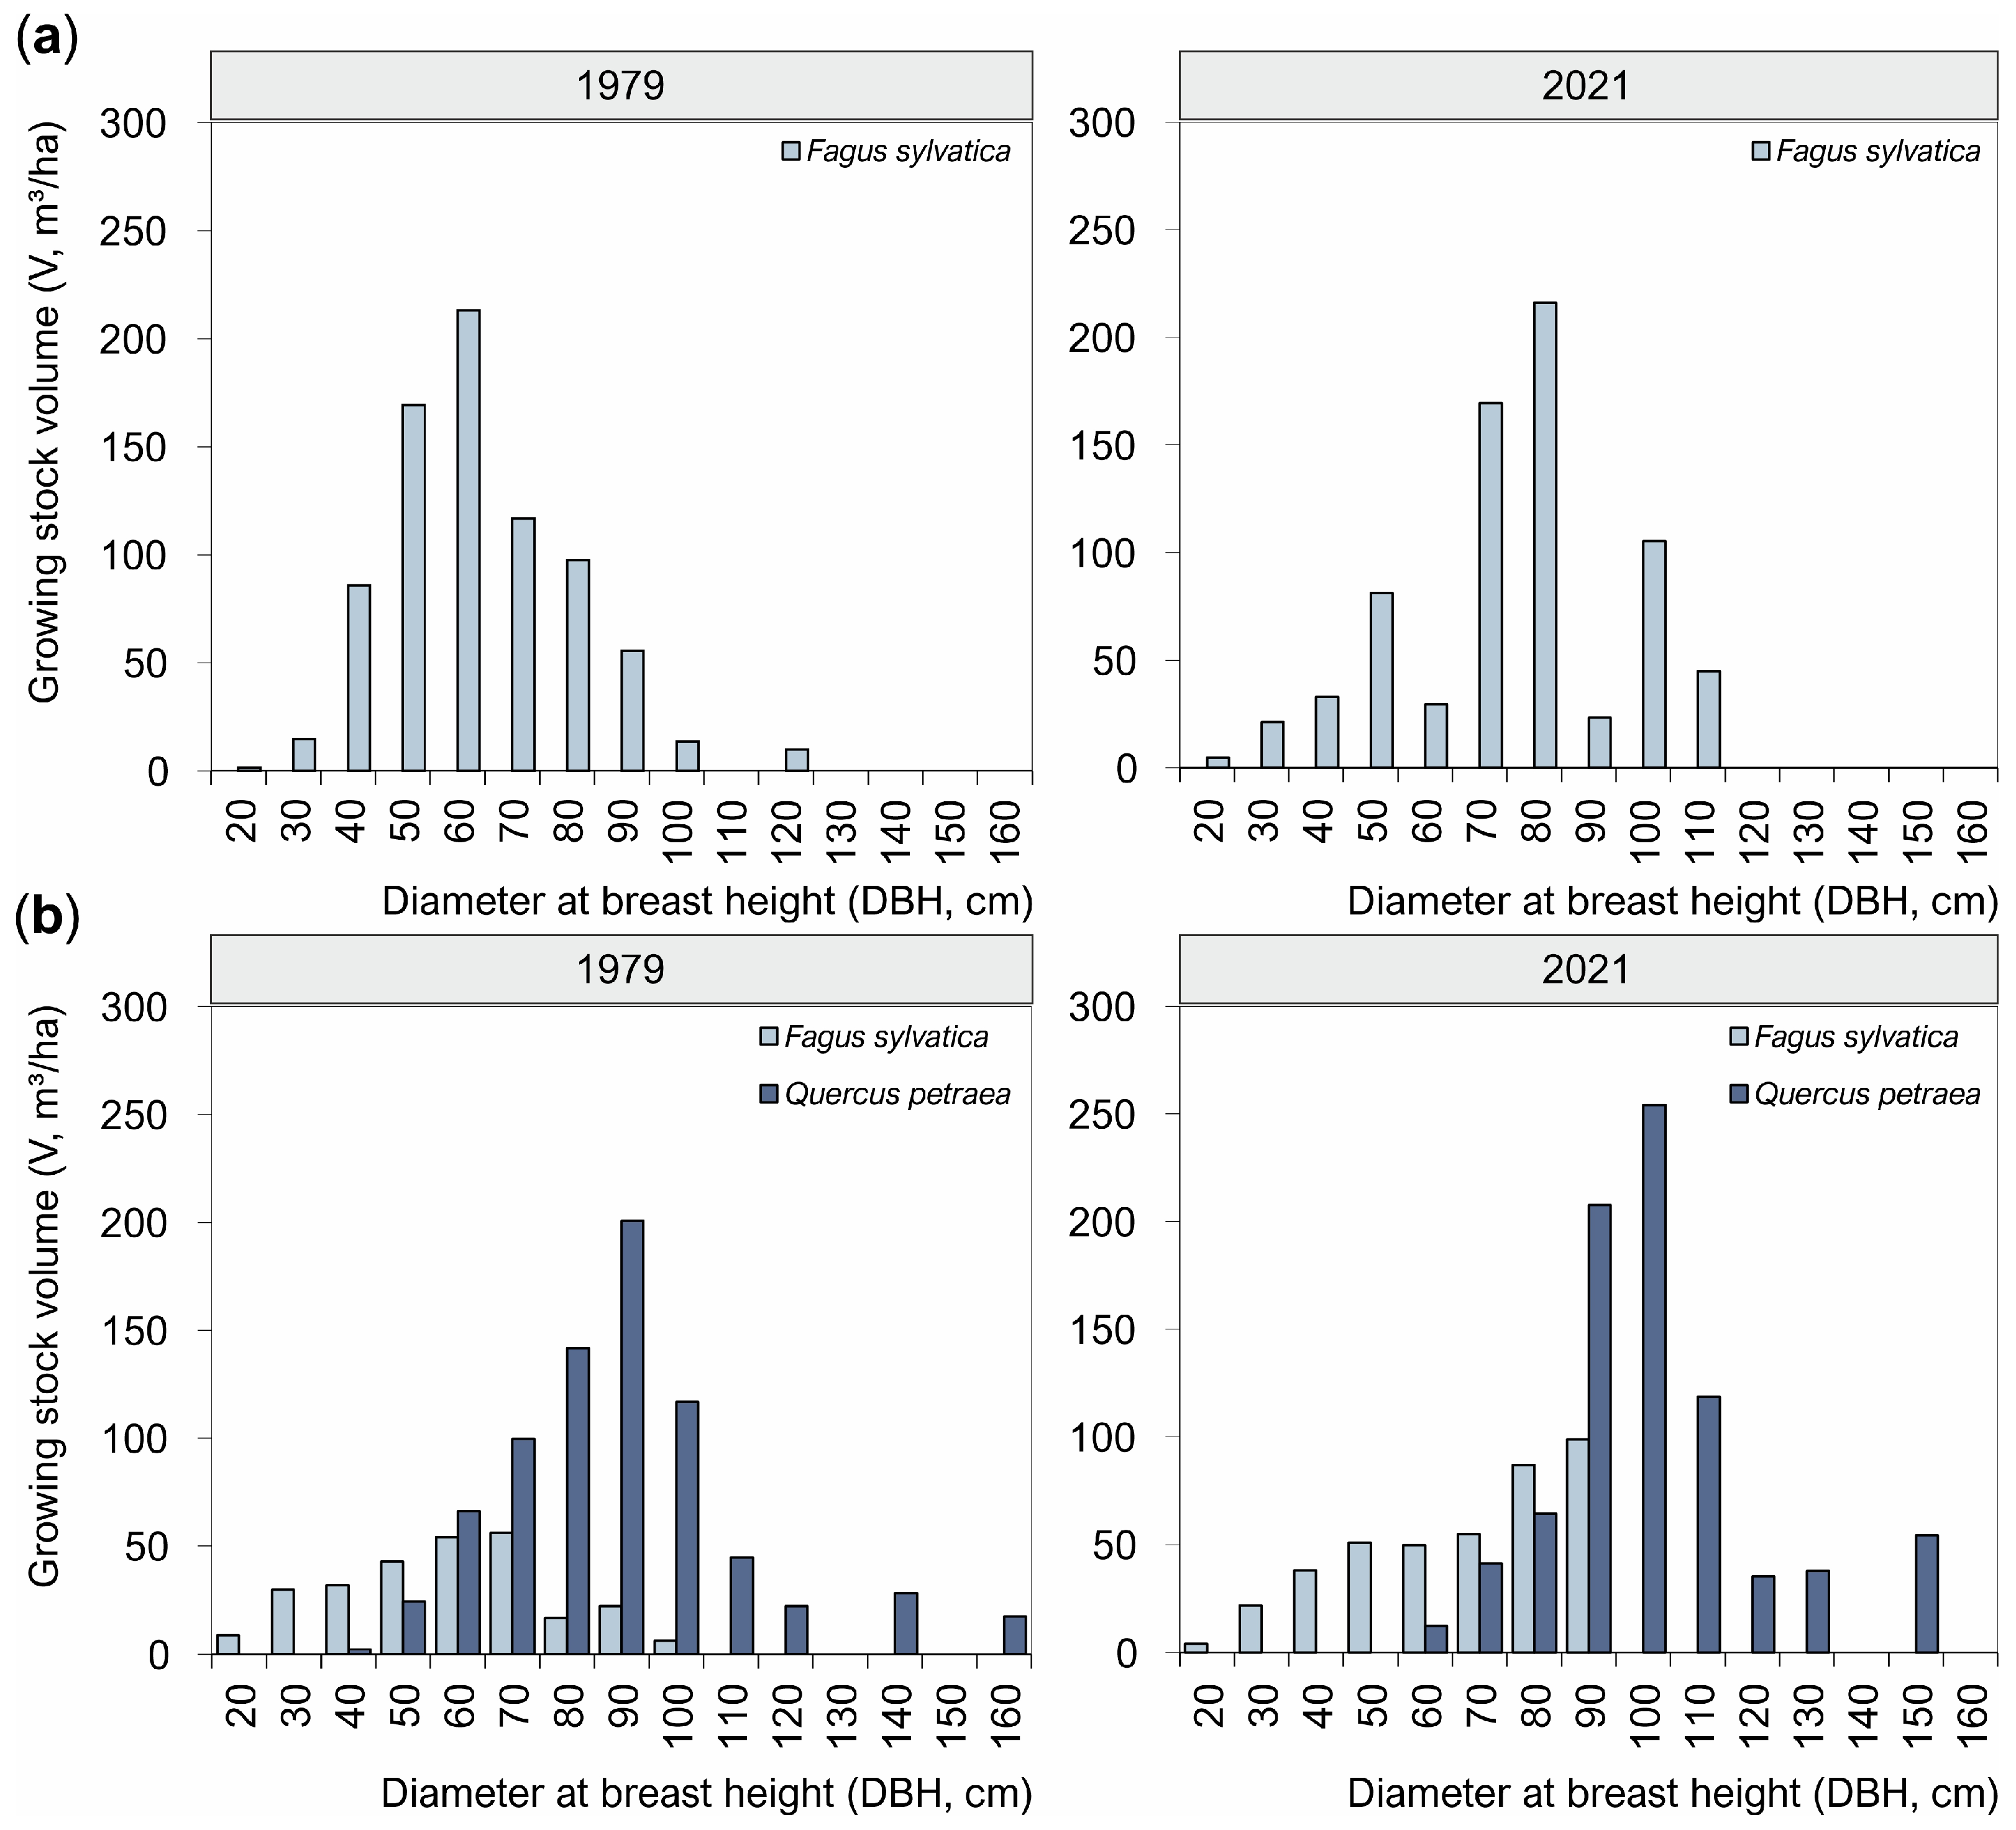
Compared to 1979, tree density decreased for both species, from 202 to 153 trees ha−1 in beech and from 94 to 73 trees ha−1 in oak. This was accompanied by an increase in growing stock volume, particularly in oak (from 776.25 to 825.55 m3 ha−1), while beech volume also increased (from 268.53 to 404.77 m3 ha−1). In both stands, the majority of growing stock was concentrated in medium and larger diameter classes, with a clear shift toward larger diameters over the study period. In the pure beech stand, volume was mainly concentrated in intermediate diameter classes, whereas in the mixed stand it was predominantly associated with larger diameter classes (Figure 4).
Figure 4.
Distribution of growing stock volume across diameter classes by species in (a) pure beech stand and (b) mixed sessile oak–beech stand for the 1979 and 2021 inventories.
3.2. Age Structure
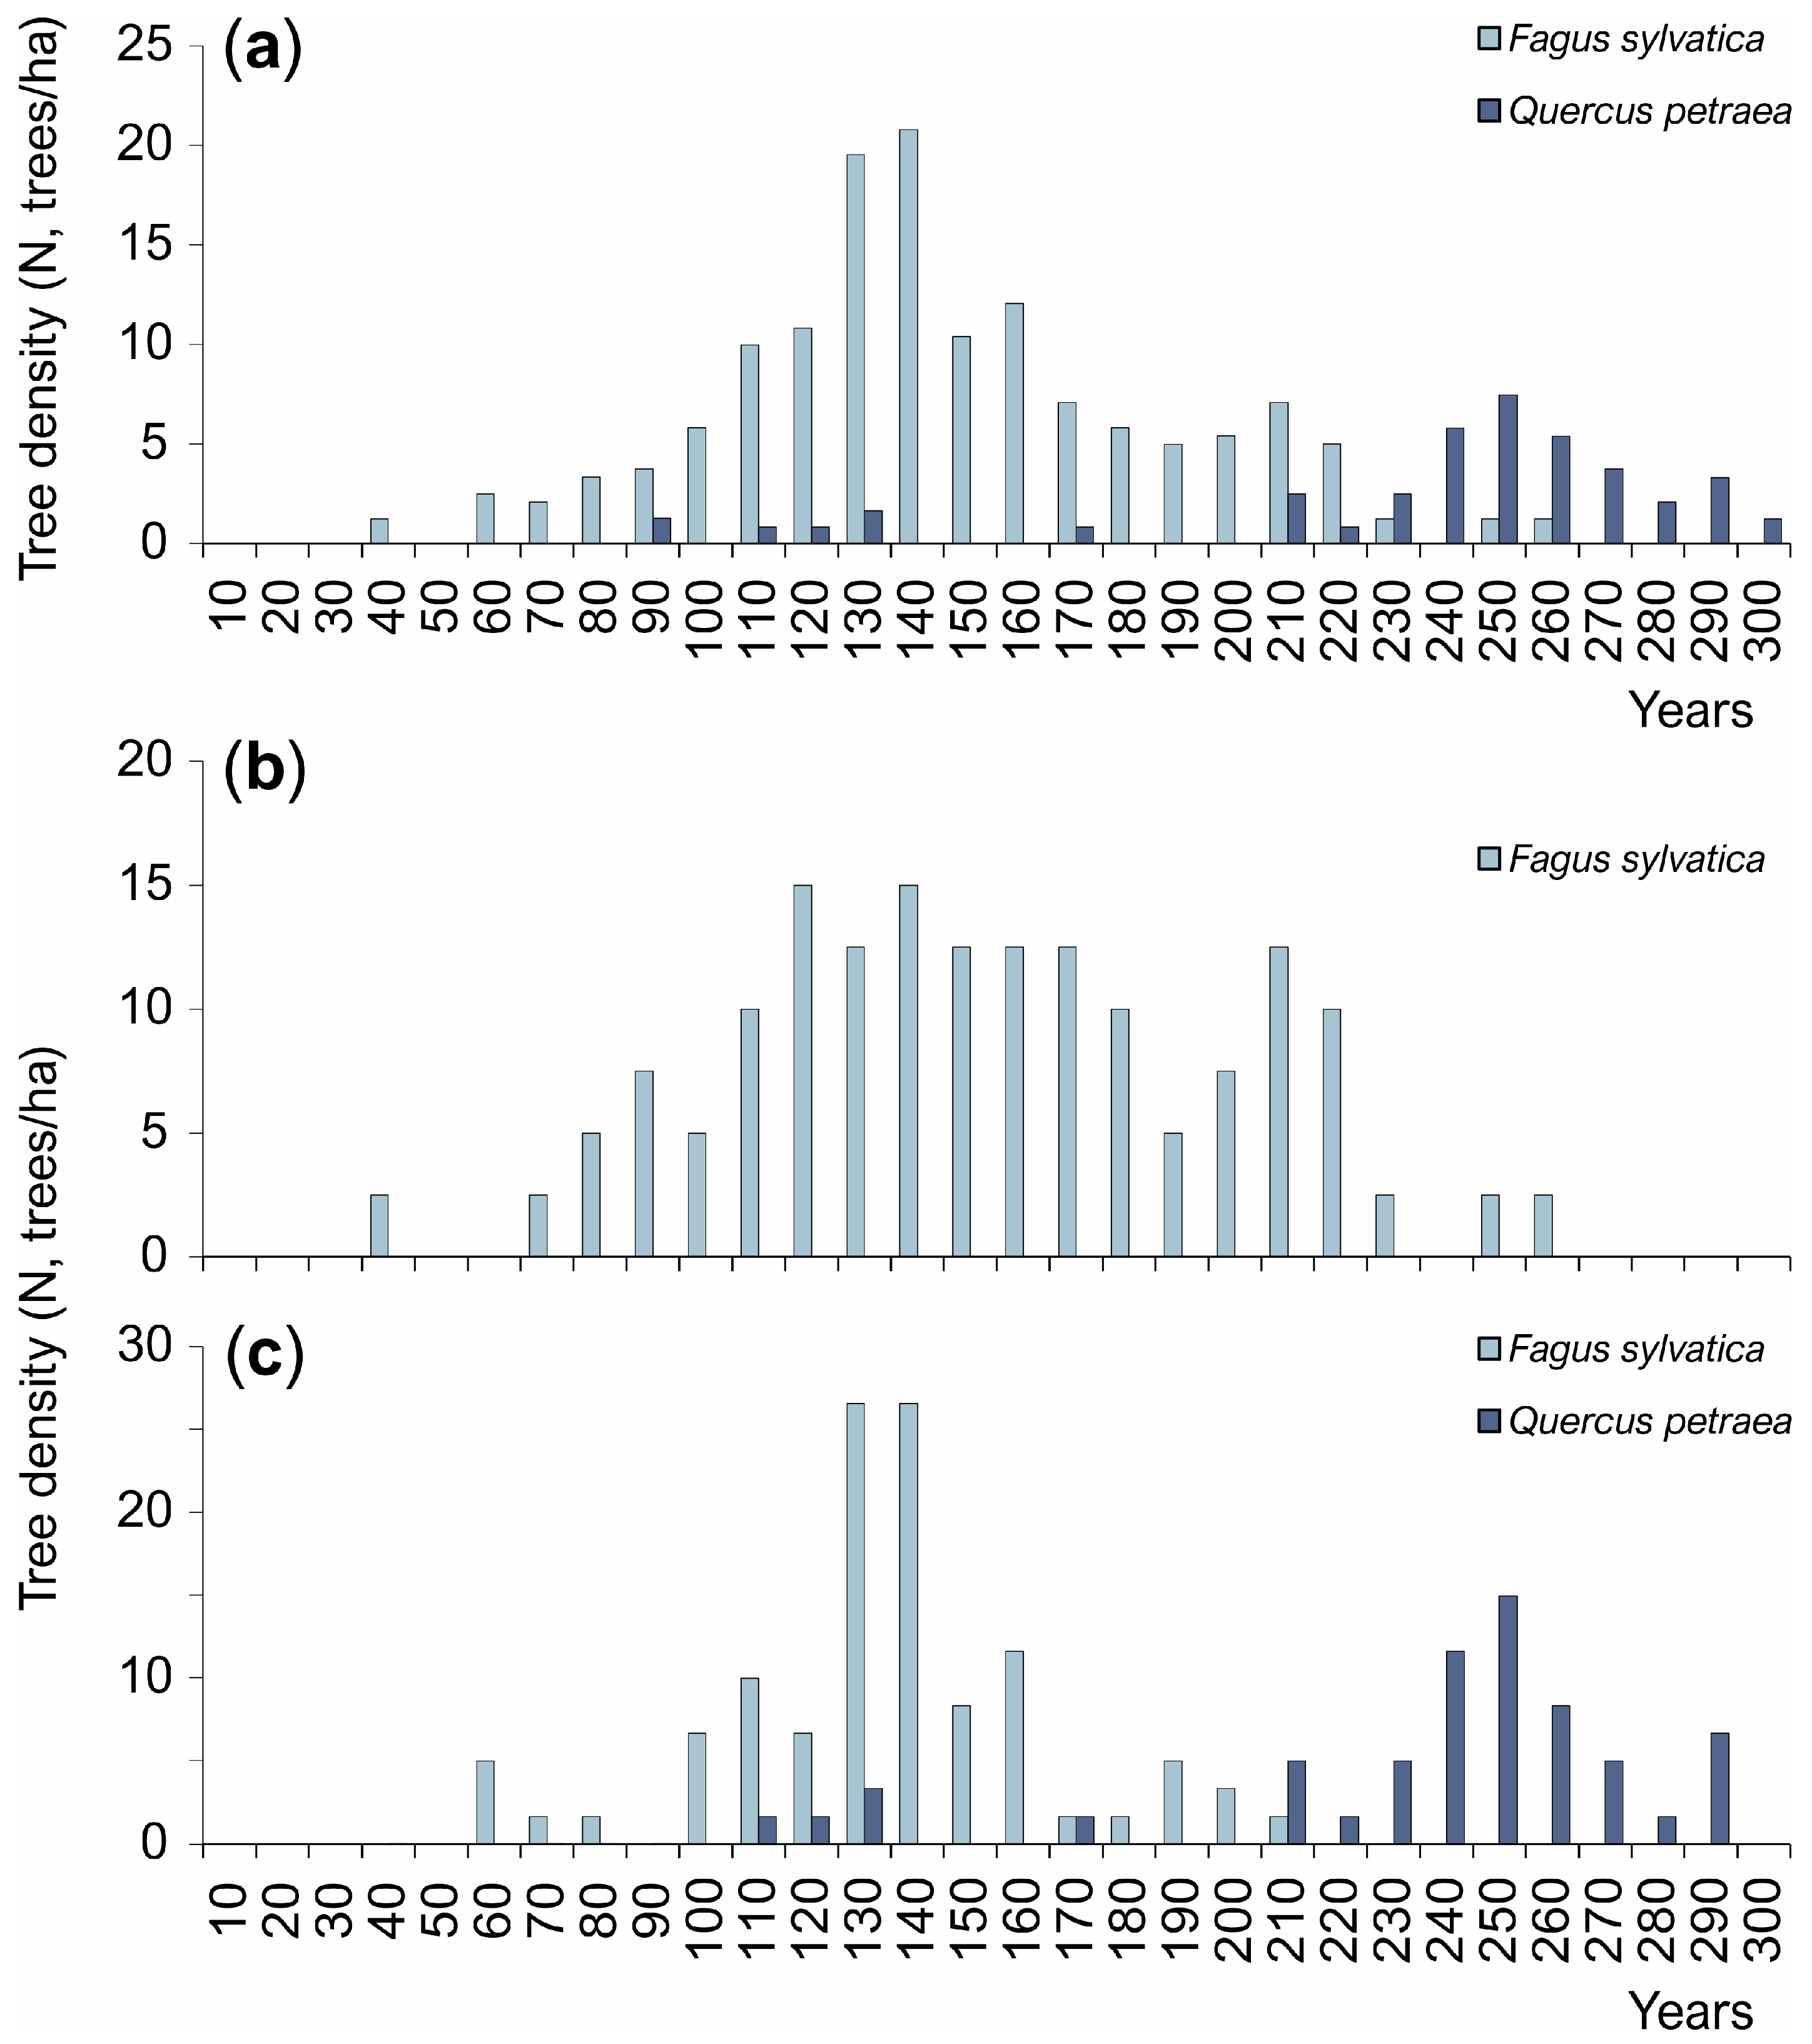
Analysis of age structure based on a sample of 197 trees revealed pronounced differences between beech and oak. Sessile oak ranged in age from 87 to 295 years, with a mean age of 252 years, whereas beech reached a maximum age of 254 years with a mean of 126 years. Beech was present across nearly the entire age range, from the youngest classes (10–30 years) to individuals older than 200 years, with the highest representation in intermediate age classes (110–150 years). In contrast, sessile oak was poorly represented in younger and intermediate age classes and was predominantly concentrated in older age classes, particularly above 220 years, with a peak between 250 and 270 years.
Age structure differed clearly between the pure beech stand (Figure 5b) and the mixed beech–oak stand (Figure 5c). In the pure beech stand, the age distribution was continuous, with the highest representation in intermediate age classes (110–170 years), indicating ongoing regeneration and the presence of multiple cohorts. In the mixed beech–oak stand, age structure was more distinctly differentiated between species. Beech dominated younger and intermediate age classes (100–160 years), whereas oak was concentrated in older age classes, most commonly between 220 and 280 years. This reflects a clear separation of age cohorts between the two species. Overall, the age structure indicates a multi-cohort system, with beech present across a wide age range and oak largely confined to older age classes.
Figure 5.
Distribution of tree age classes (10-year intervals) for (a) the entire reserve, (b) pure beech stand and (c) mixed sessile oak–beech stand.
3.3. Results of Canopy Gap Analysis
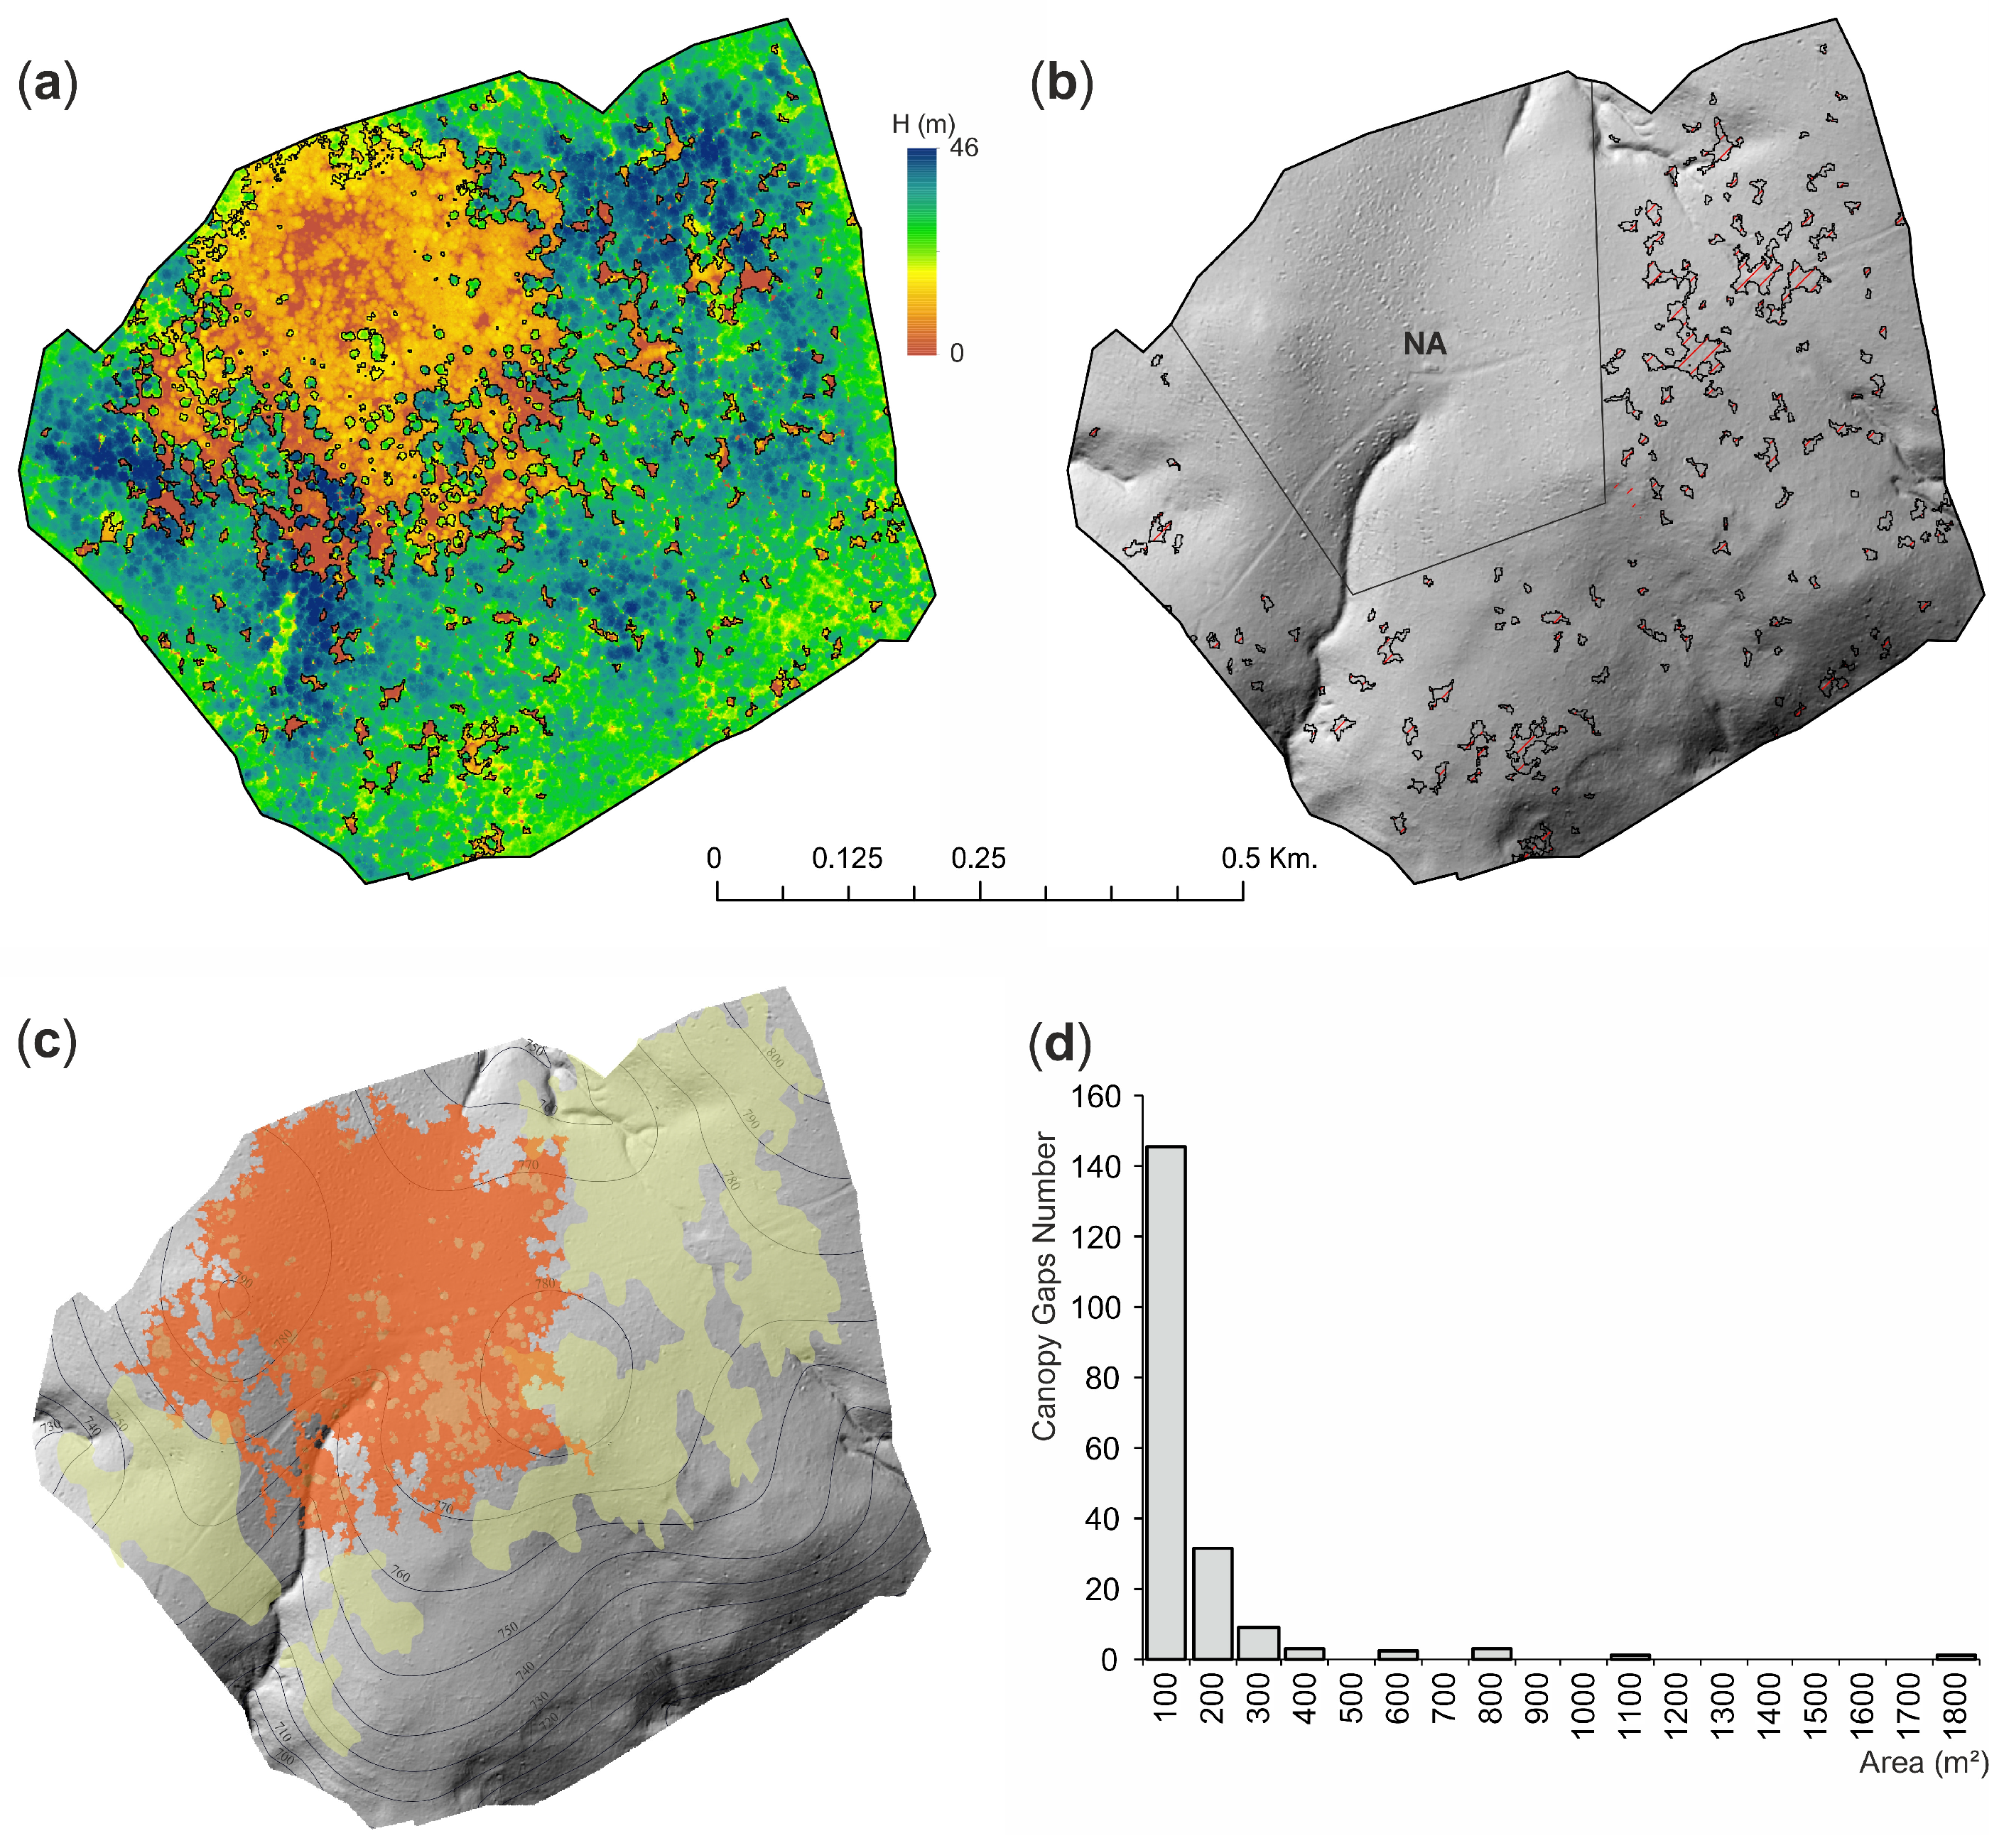
Canopy gap analysis in the Muški bunar old-growth forest was conducted over an area of 36 ha, excluding the section affected by the 1999 windthrow (Figure 6a). A total of 195 canopy gaps were identified, covering 21,105 m2, which corresponds to approximately 5.9% canopy openness and an average of 5.4 gaps ha−1 (Figure 6b). The mean gap size was 108.2 m2, with a median of 59 m2 and a modal value of 29 m2. Gap sizes ranged from 25 m2 to 1716 m2, with a high standard deviation (176.6 m2) and coefficient of variation (163%) (Figure 6d).
Figure 6.
Canopy height model (CHM) of the Muški bunar old-growth forest in 2021 (a); detected canopy gaps excluding areas affected by the 1999 windthrow (b); spatial extent of windthrow disturbances in 1999 (orange) and 2023 (yellow) (c); and distribution of canopy gap sizes (d). NA indicates areas excluded from the analysis due to the 1999 windthrow disturbance.
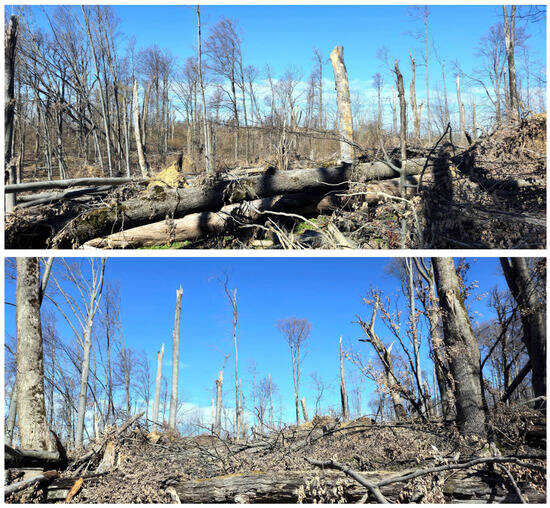
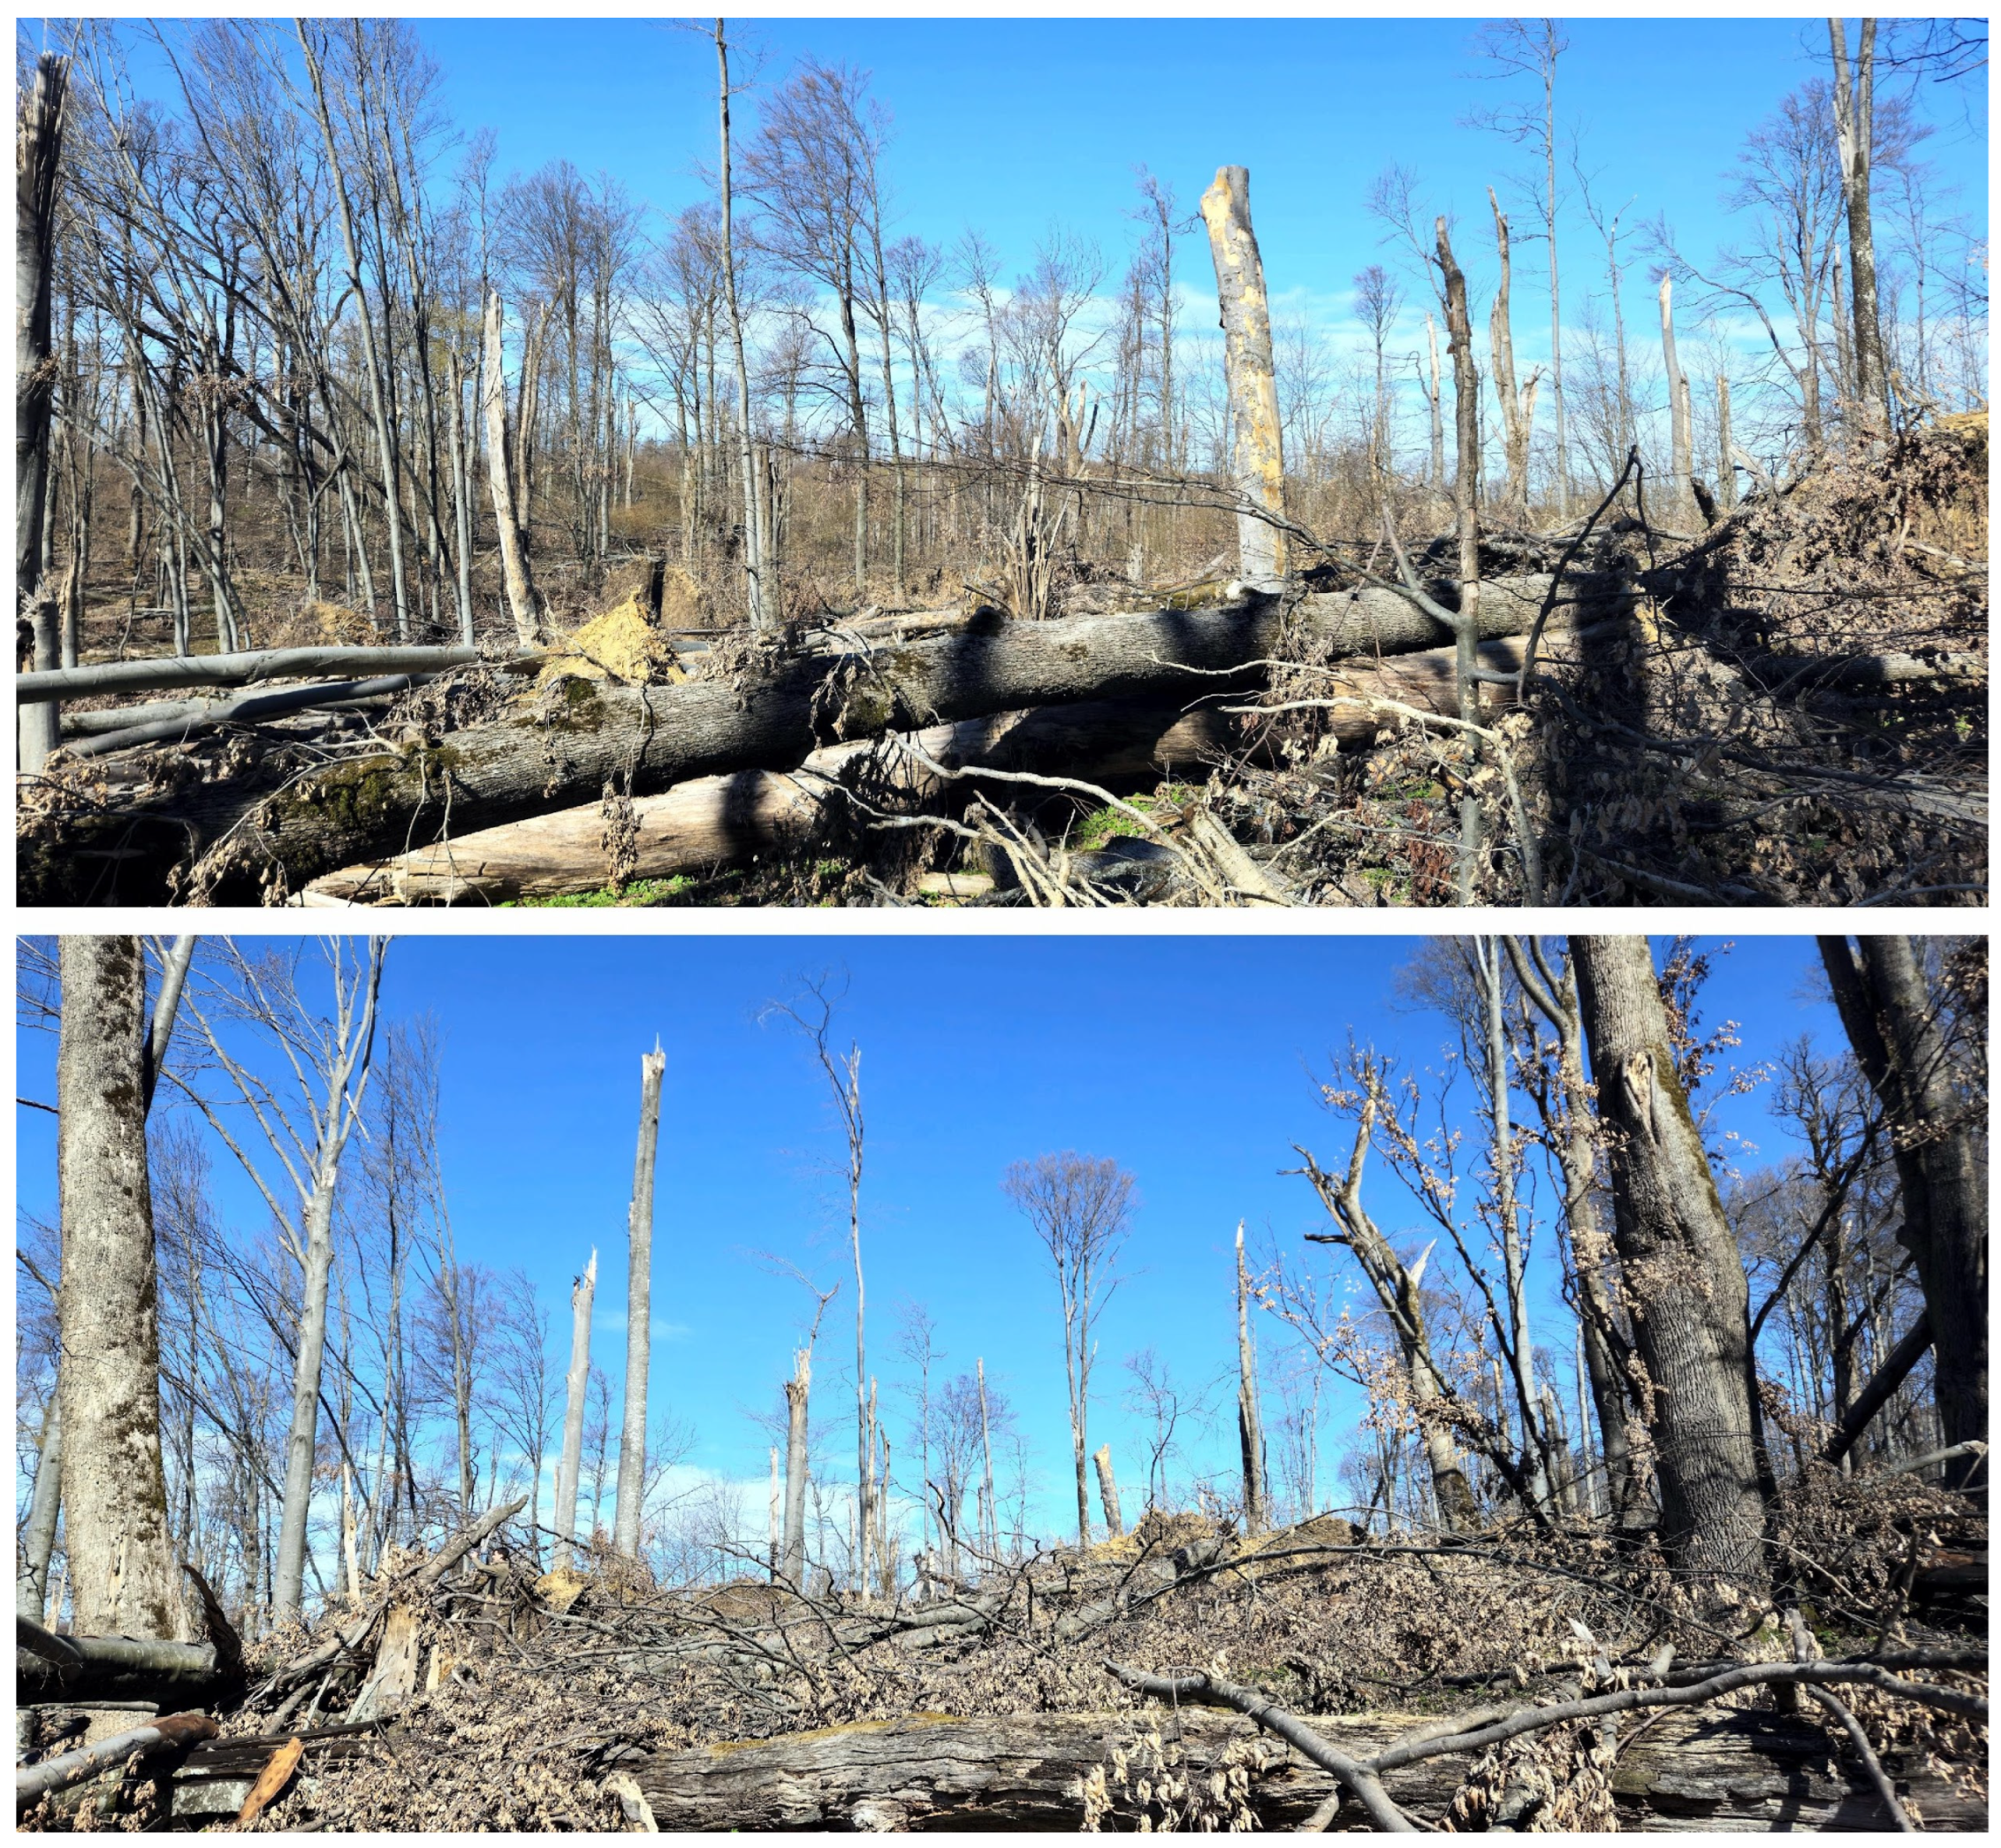
In addition to the dominance of small canopy gaps (Figure 6), two high-intensity disturbance events were recorded in the reserve, namely windthrows in 1999 and 2023. On 21 June 1999, a severe storm affected the western Psunj massif, causing substantial damage to surrounding forest stands as well as within the reserve. Approximately 5760 m3 of timber was damaged over an area of 9.6 ha. The reserve was affected again by a storm event on 19 July 2023 (Figure 7), during which an estimated 11,520 m3 of timber was damaged over an area of up to 14.4 ha. This estimate is based on a post-disturbance field inventory conducted by Hrvatske šume d.o.o., the state-owned forest management company responsible for the study area. Both disturbance events primarily impacted the part of the reserve dominated by European beech (Fagus sylvatica), while the mixed beech–oak stand remained largely unaffected. Prior to these events, no disturbances of such magnitude had been recorded in the reserve.
Figure 7.
Windthrow disturbance events in Muški bunar 2023 (photo: S. Mikac).
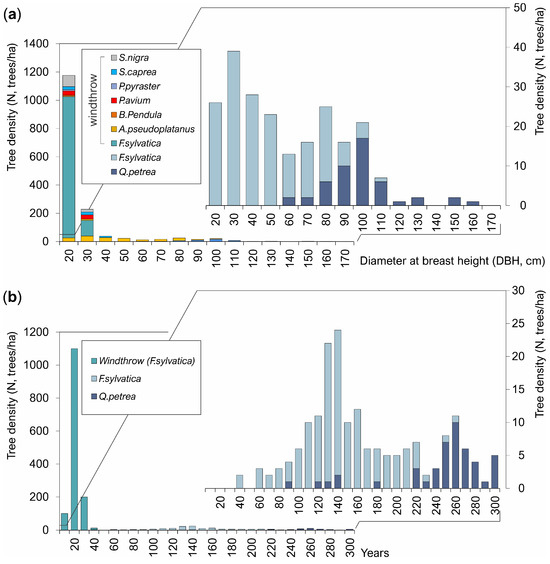
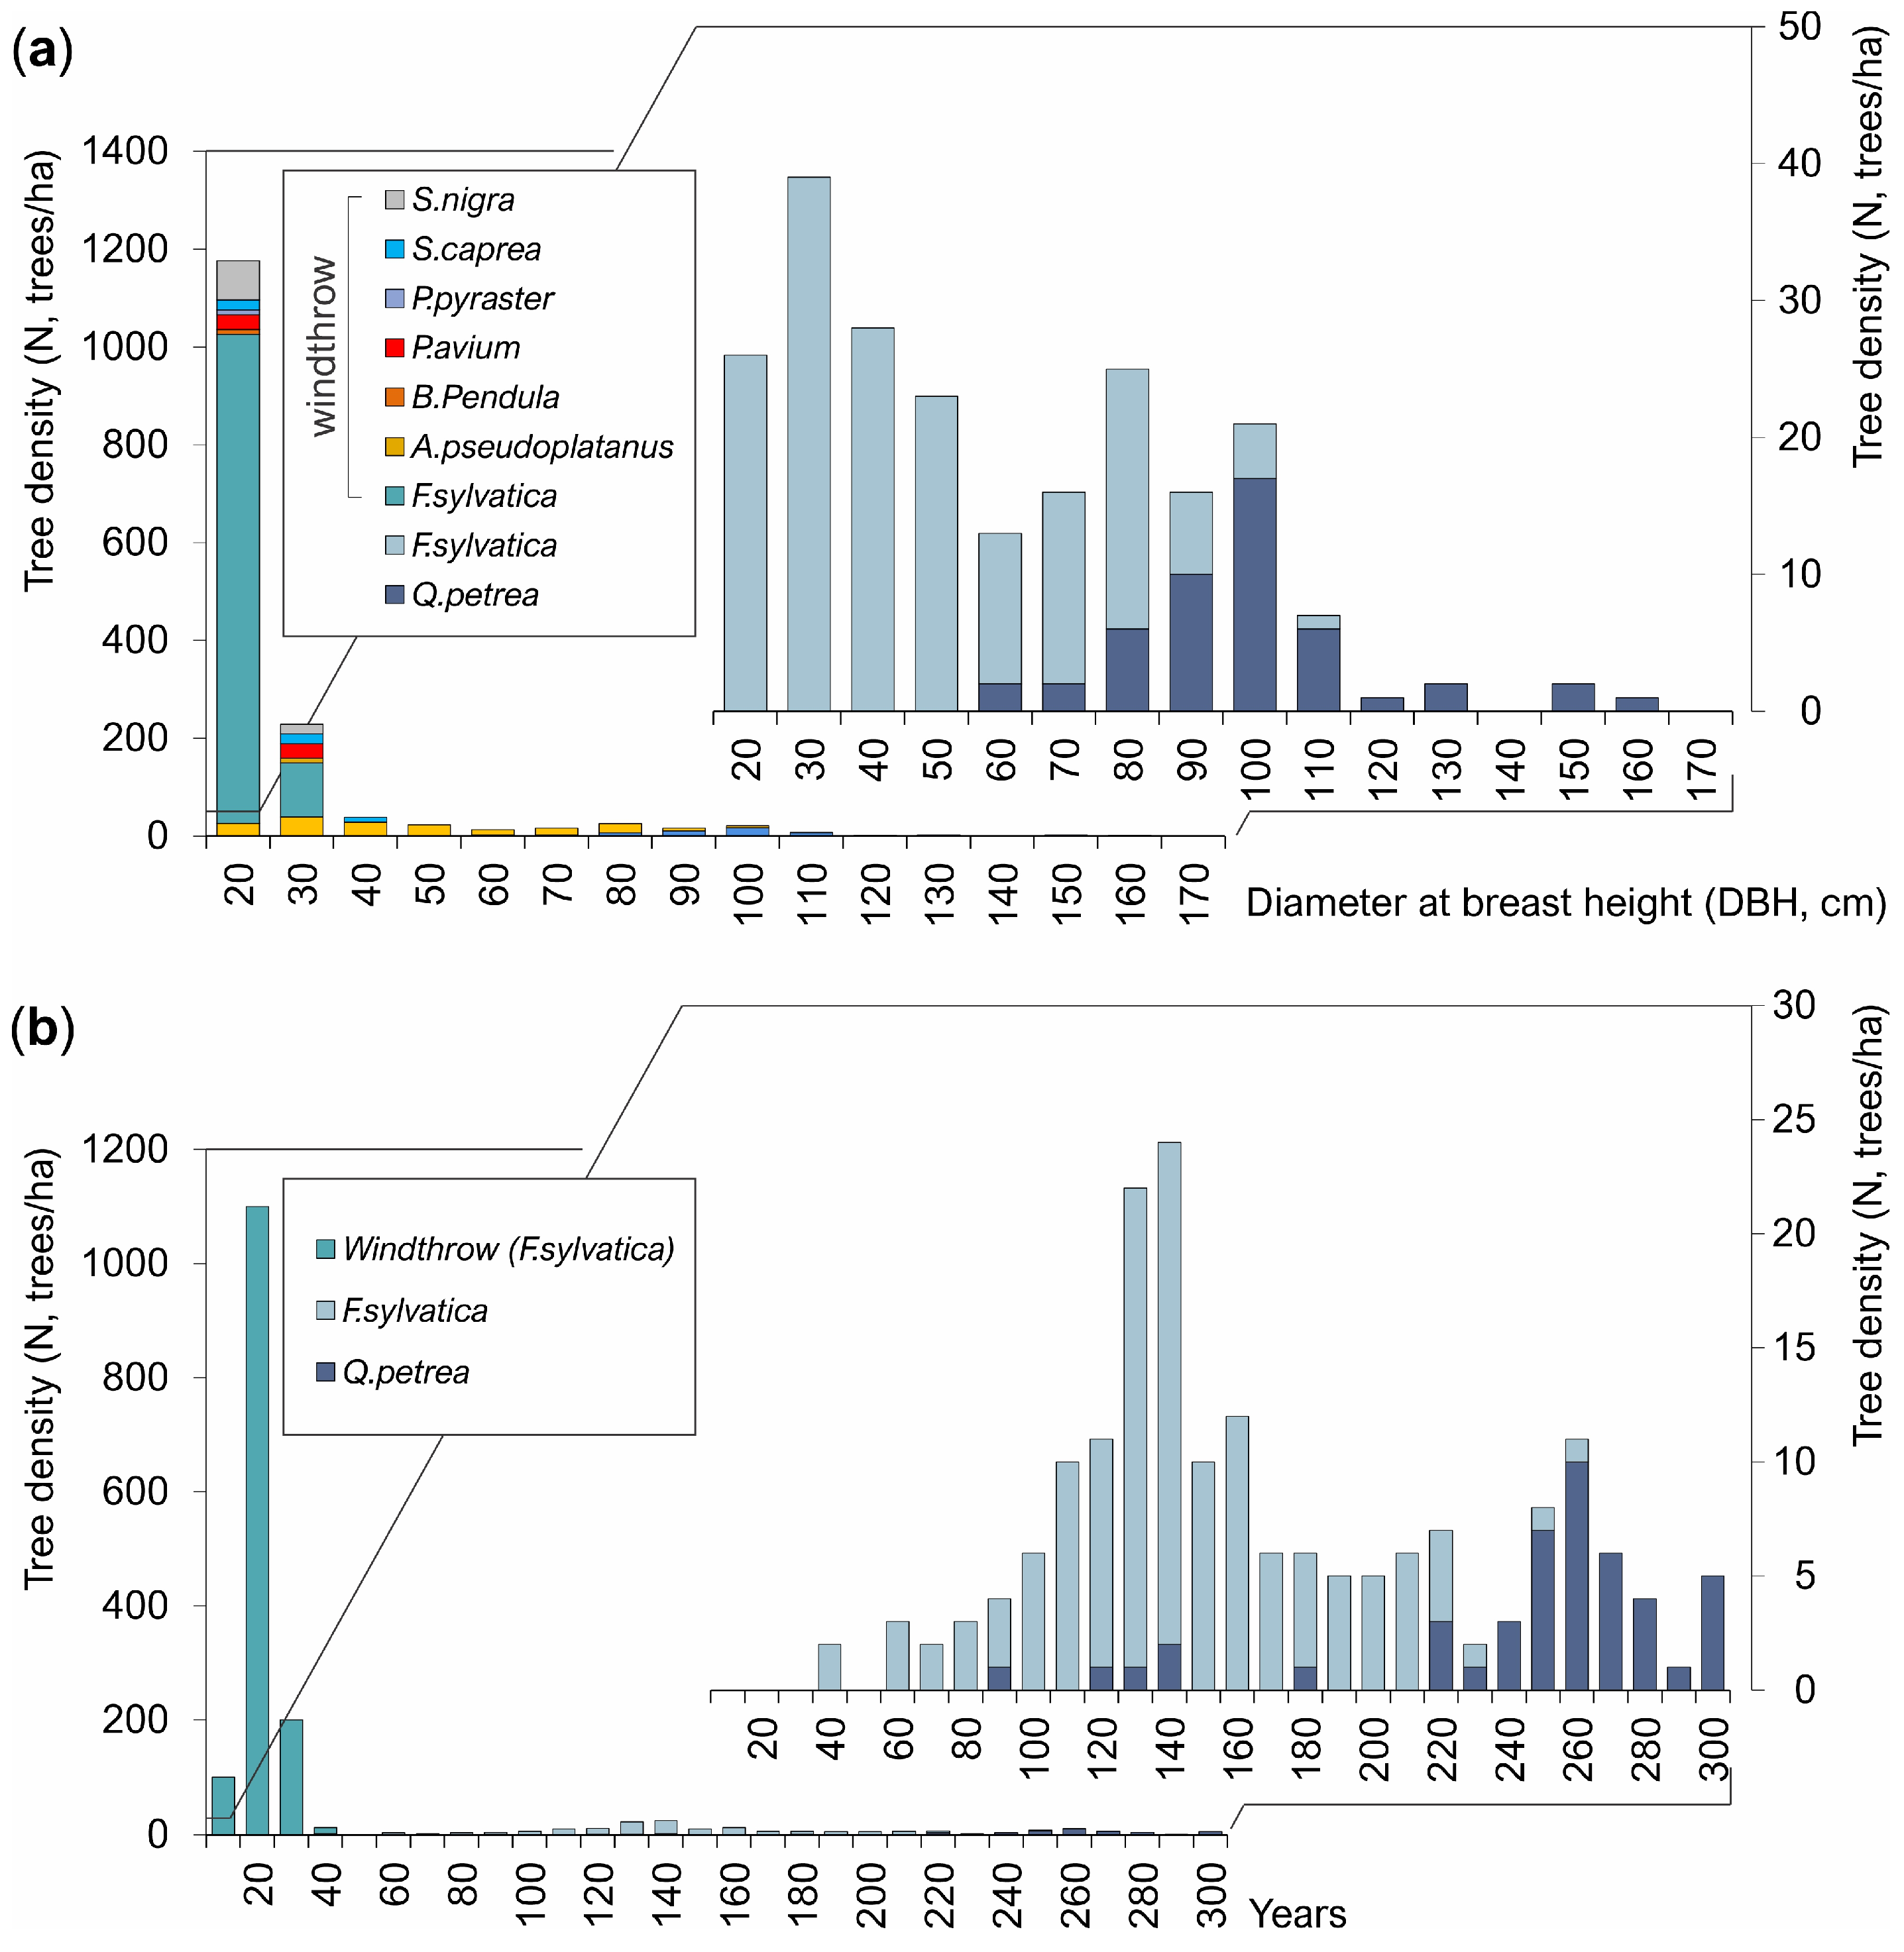
In the area affected by the 1999 windthrow, a very dense young stand dominated by beech was recorded 23 years after the disturbance. The stand successfully regenerated through natural regeneration, with a beech density of 1120 trees ha−1, a mean diameter at breast height of 14.0 cm (Figure 8a), and an average tree height of approximately 10 m. In addition to beech, several other tree and shrub species were recorded within the windthrow area, including sycamore maple (Acer pseudoplatanus L.), silver birch (Betula pendula Roth), wild cherry (Prunus avium (L.) L.), wild pear (Pyrus pyraster (L.) Burgsd.), goat willow (Salix caprea L.), and elder (Sambucus nigra L.). A total of 1340 individuals ha−1 were recorded, with beech accounting for the dominant share of 82.8%, while the remaining species were represented in lower proportions: elder 7.5%, wild cherry 4.5%, goat willow 3.7%, and sycamore maple, silver birch, and wild pear each accounting for 0.7%. The remaining species collectively accounted for approximately 17.2% of the total number of individuals, indicating the presence of accompanying and pioneer species in the early stage of stand development following disturbance.
Figure 8.
Distribution of the number of trees across diameter classes and tree species for the entire reserve (a) and distribution of the number of trees across age classes (b), including the area affected by the 1999 windthrow. For better visualization and to highlight the shapes of the distributions, selected parts of the graphs are enlarged.
Figure 8a shows the distribution of the number of trees across diameter classes at the level of the entire reserve, including areas affected by windthrow, while Figure 8b presents the age distribution of the same trees. A higher proportion of beech is observed in the lower diameter classes, corresponding to the increased representation of younger age classes in Figure 8b. In the medium and larger diameter classes, both beech and sessile oak are represented, which corresponds to the distribution of older age classes (Figure 8b).
3.4. Growth Release Dynamics
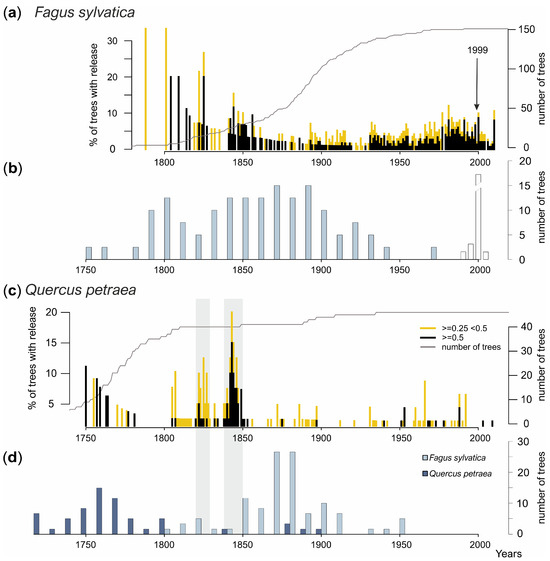
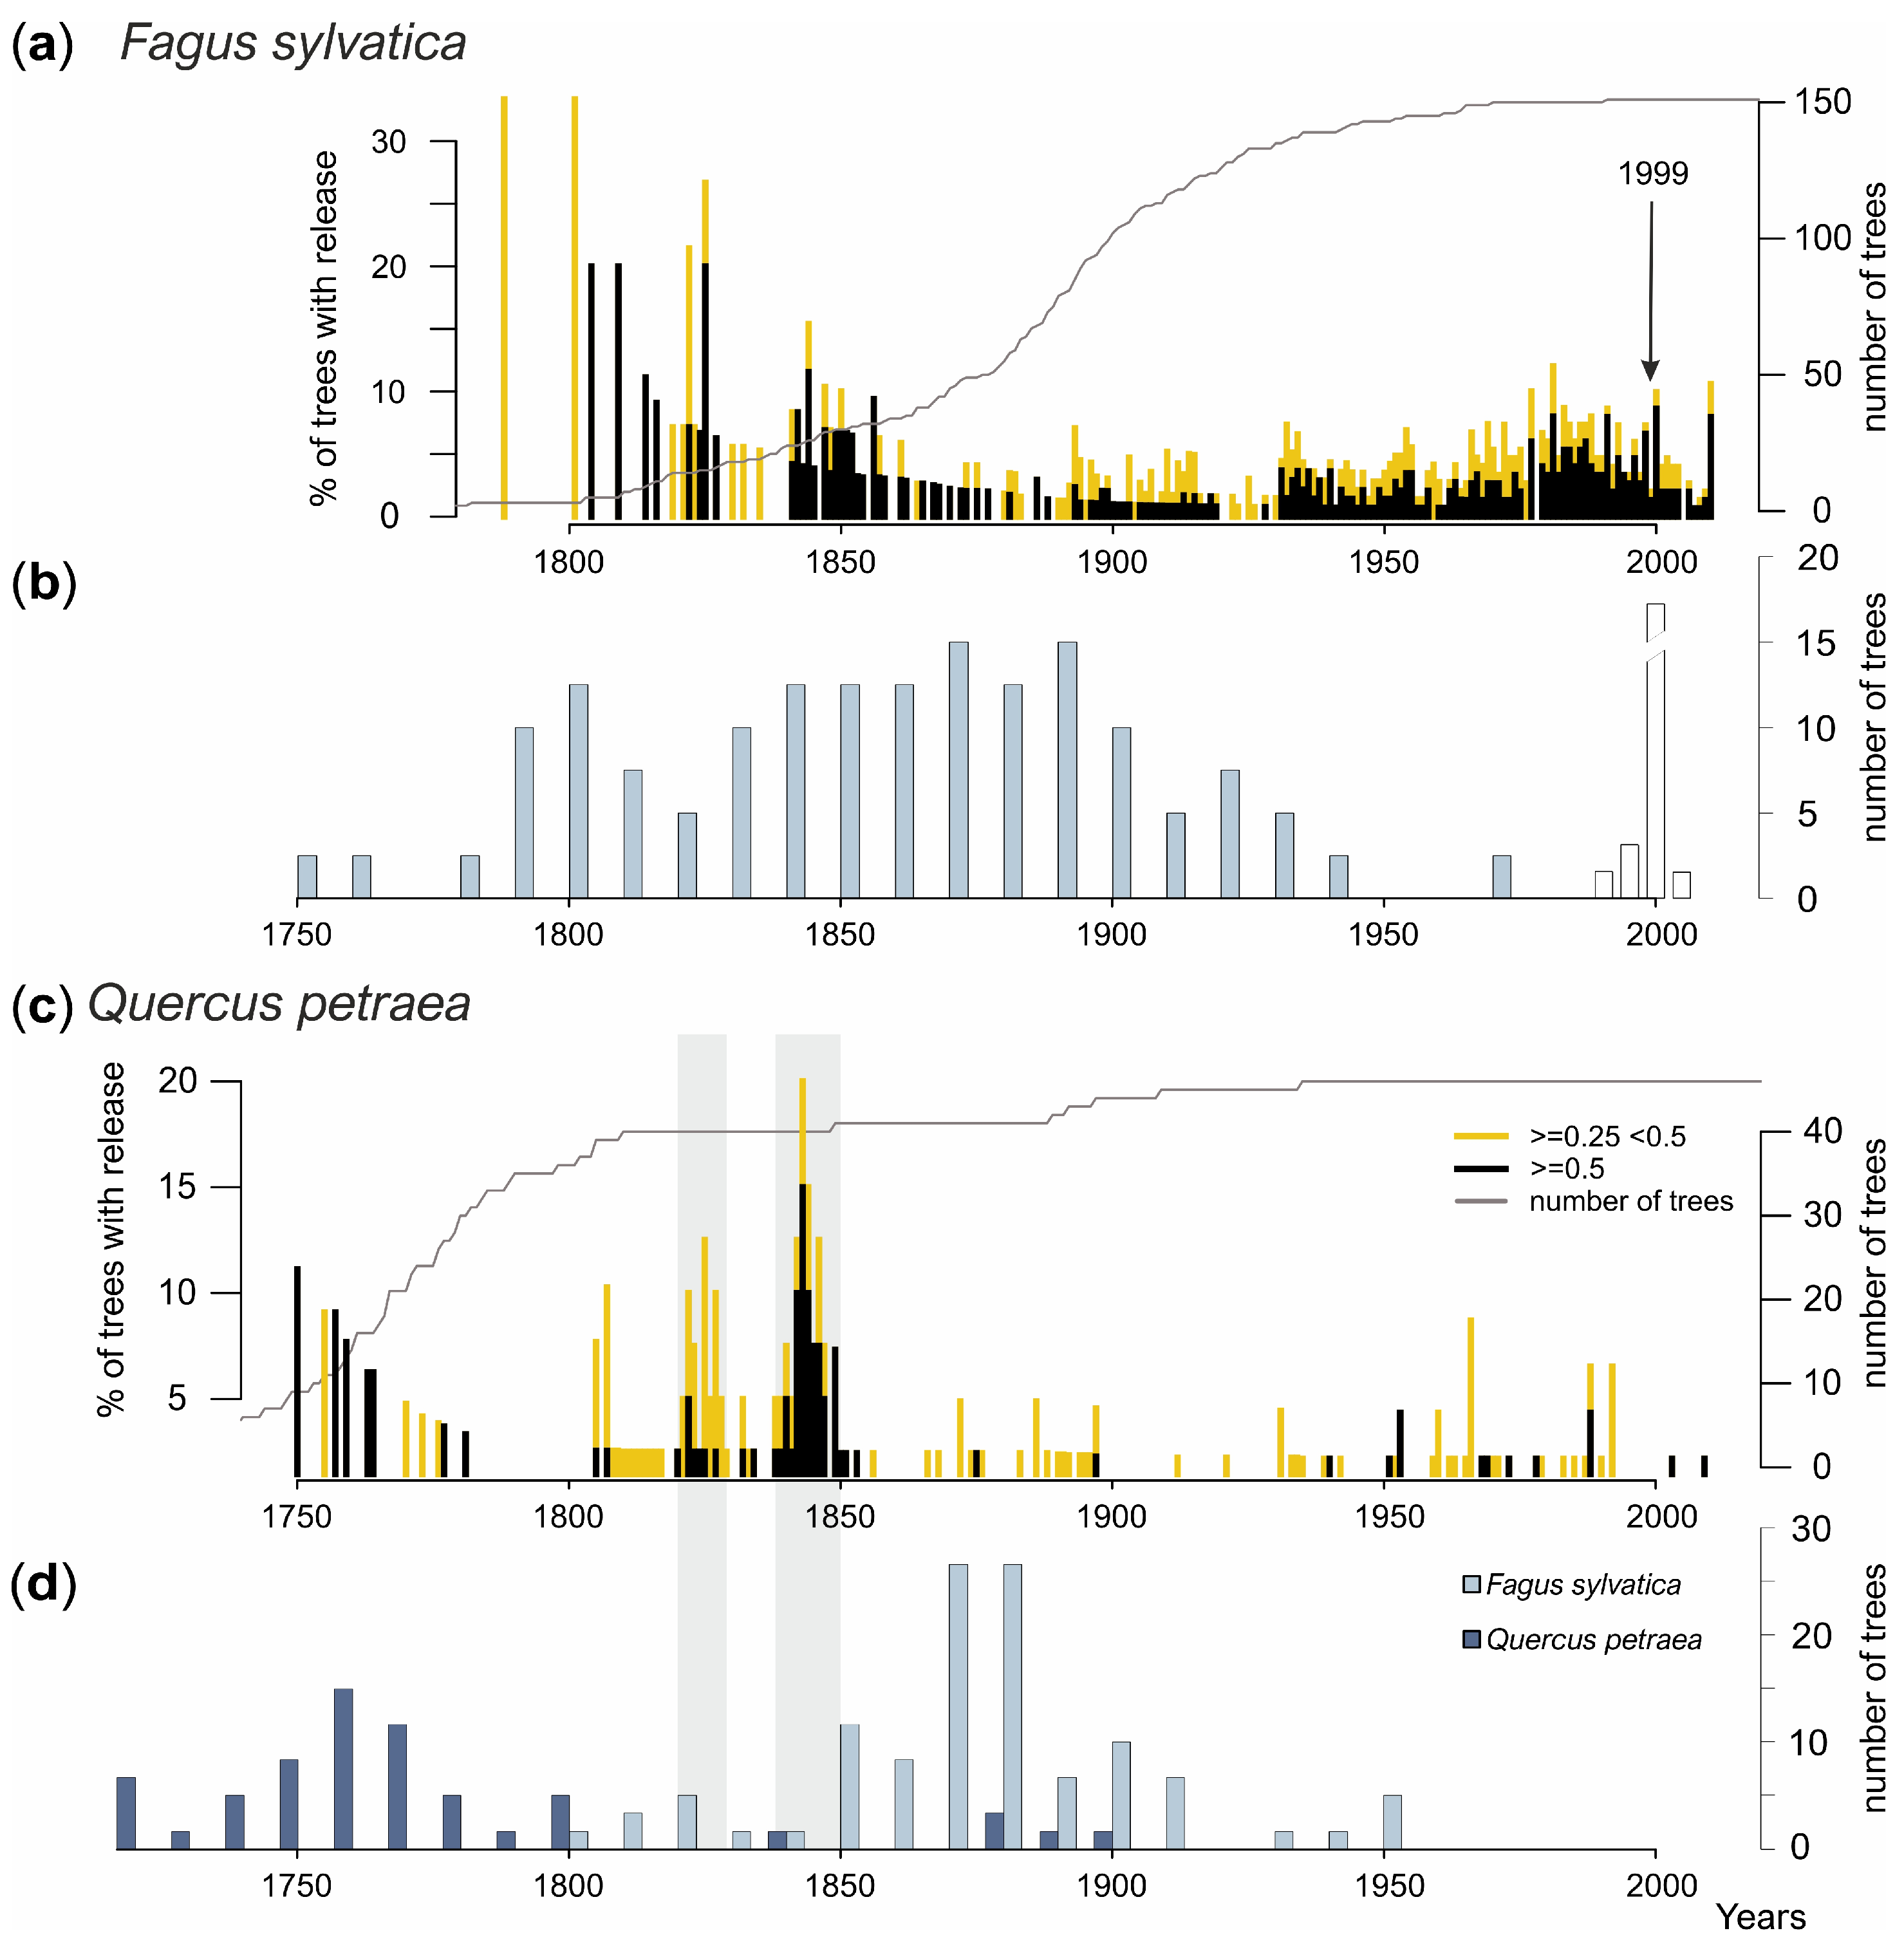
Growth release analysis revealed pronounced differences in disturbance responses between beech (Figure 9a) and sessile oak (Figure 9c). Beech exhibited a substantially higher number of growth release events (308 moderate and 399 major) compared to sessile oak (100 moderate and 65 major). The temporal distribution of growth releases in beech indicates a continuous disturbance regime, particularly pronounced during the 20th century, with frequent and prolonged periods of increased growth approximately between 1930 and 2000. In contrast to beech, oak shows a markedly different pattern characterized by strong growth release events in the 19th century, especially between 1838 and 1845. Outside this period, no significant release events were detected. Comparison with the distribution of tree establishment years shows that no regeneration of sessile oak occurred following the period of intensive growth (1838–1845), as evidenced by the absence of younger age classes (Figure 9d). In contrast, younger cohorts of European beech appeared during and after this period. The increased frequency of growth releases in beech at the end of the 20th century coincides with known high-intensity disturbance events (e.g., the 1999 windthrow) (Figure 9b).
Figure 9.
Disturbance chronology with moderate (yellow) and major releases (black bars) shown at annual resolution for beech (a) and sessile oak (c), together with the distribution of tree numbers by year of establishment for beech (b) and sessile oak (d). Grey shaded areas indicate periods of increased disturbance intensity.
3.5. Basal Area Increment
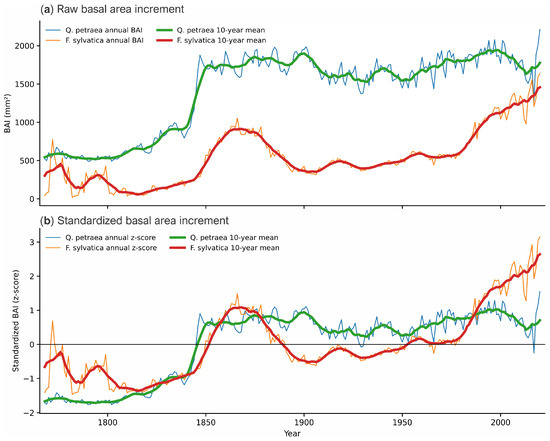
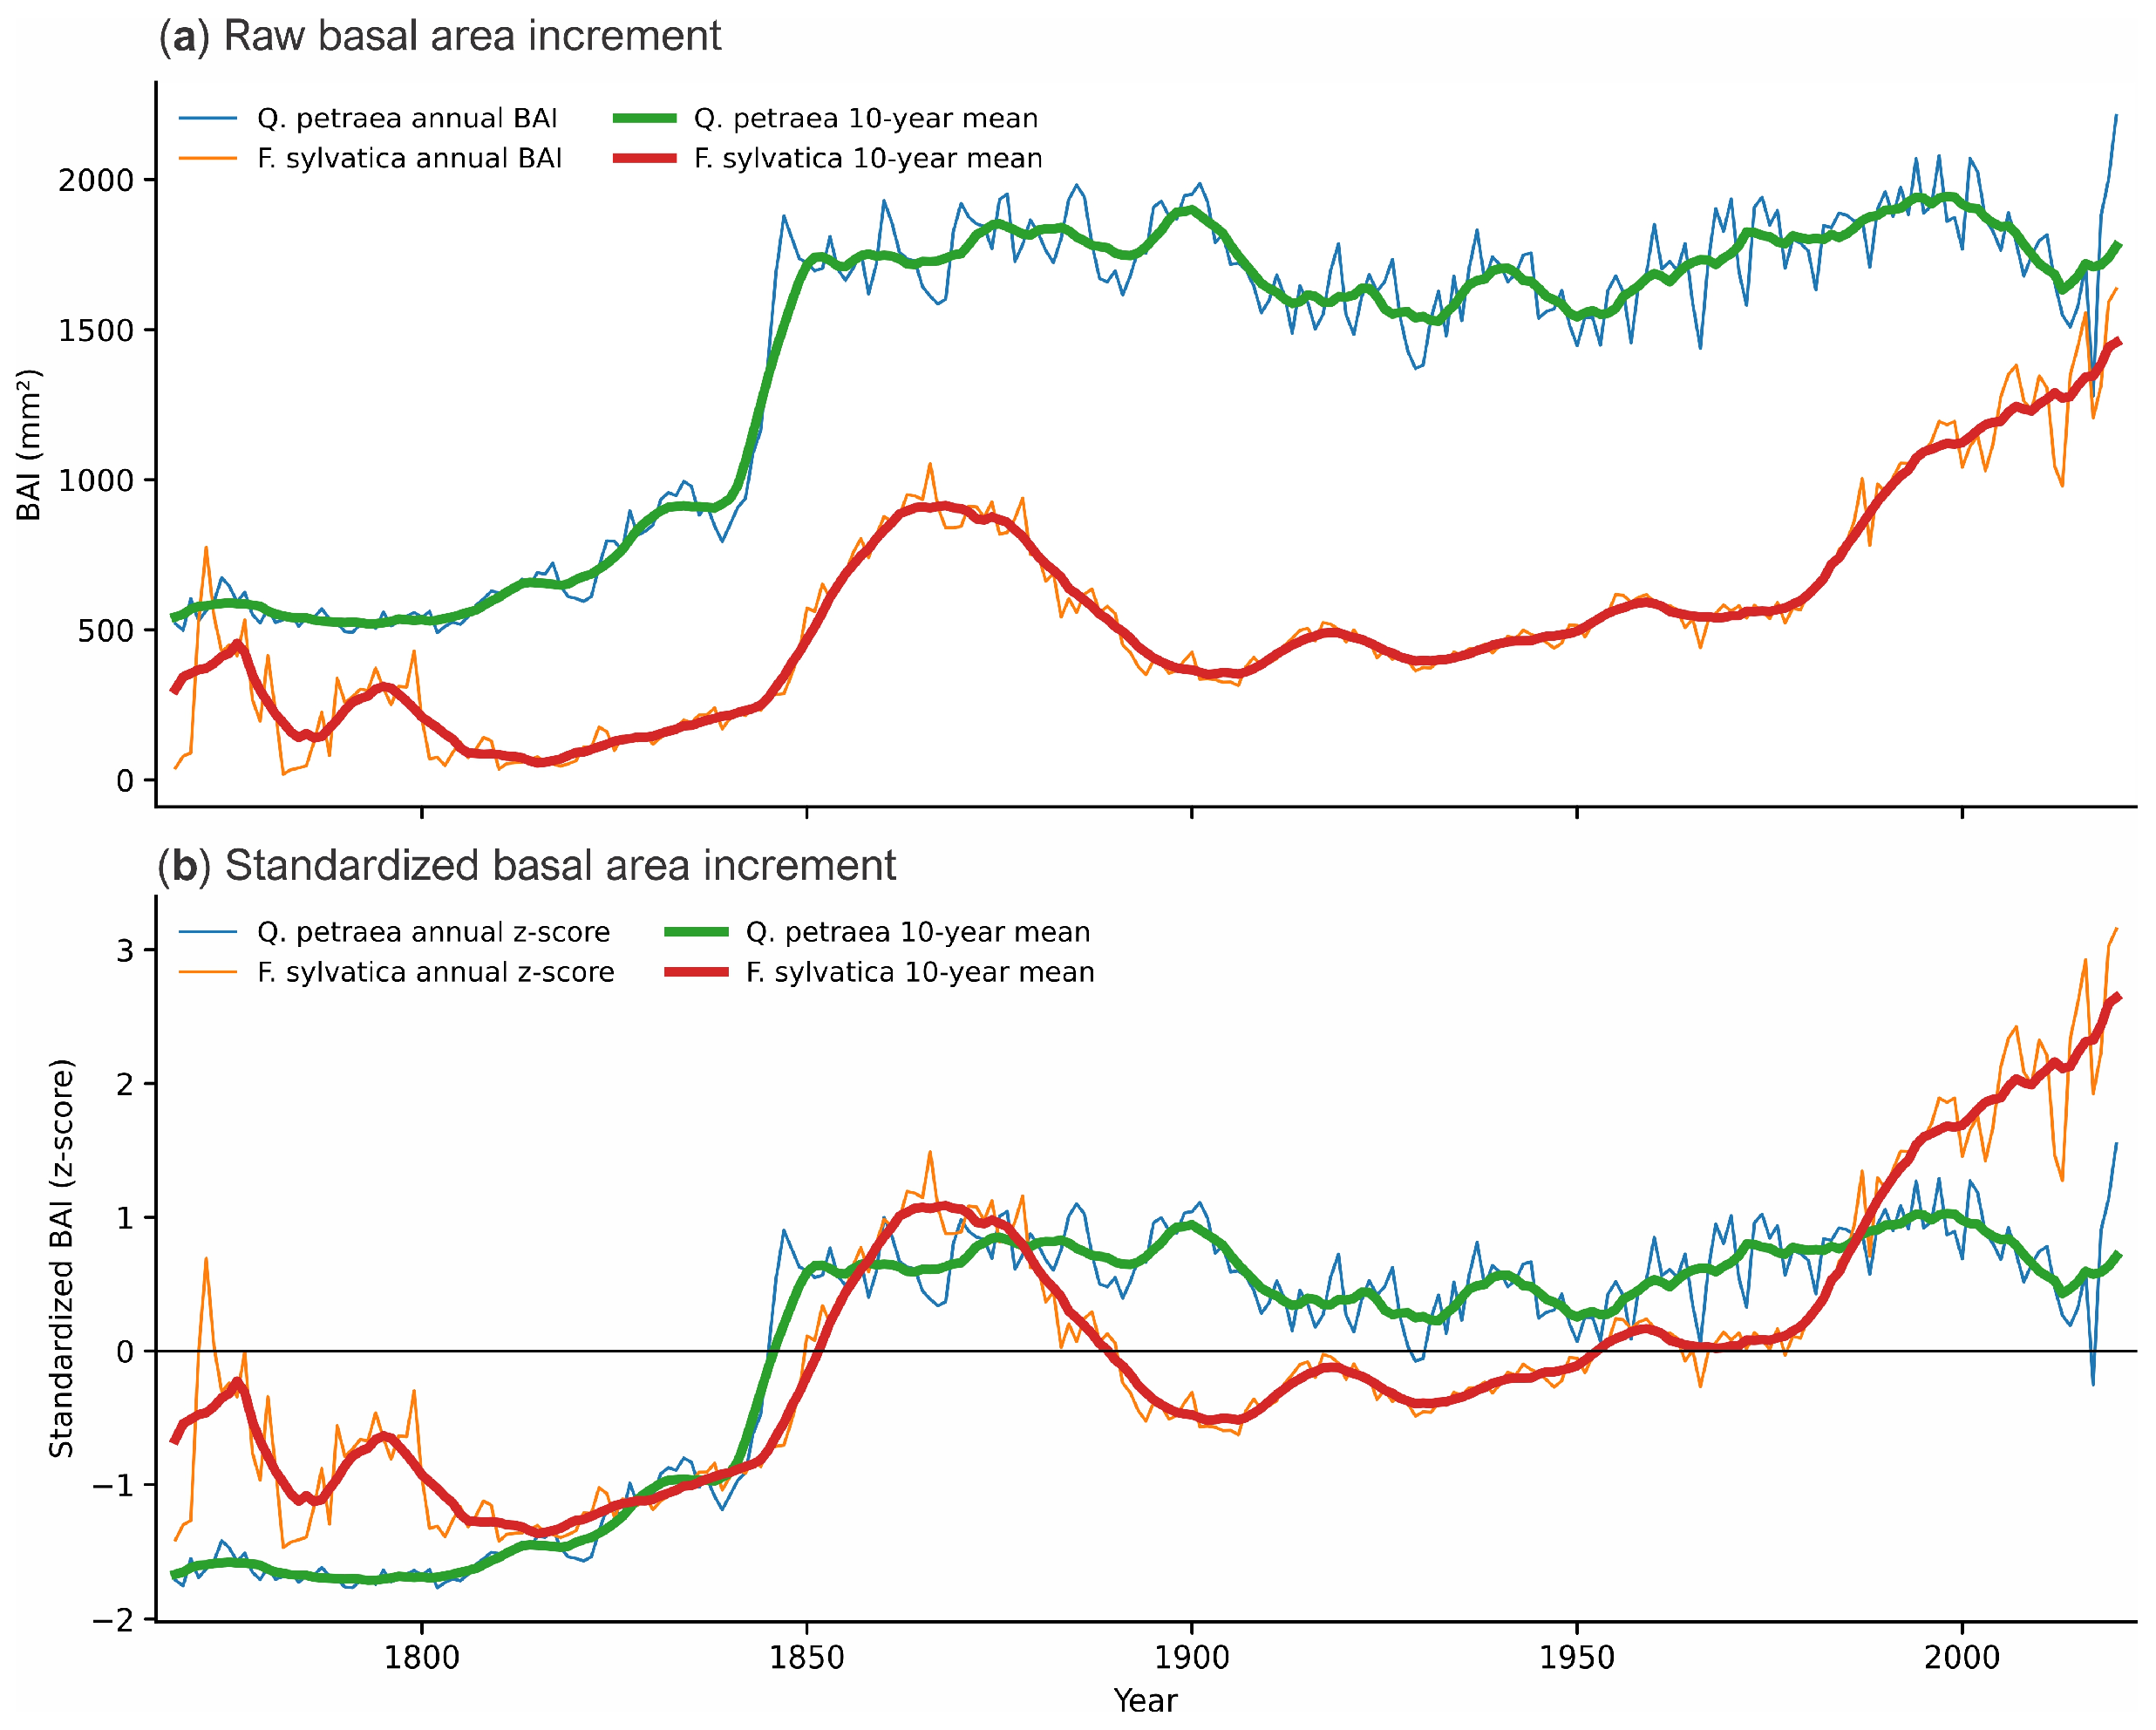
A total of 151 tree-ring width series of beech and 46 series of oak were analysed. The mean series length was 136 years for beech and 237 years for oak. The oldest beech series began in 1768, whereas the oldest oak series dated back to 1727. Mean ring width was 1.254 mm for beech and 1.385 mm for oak. Mean sensitivity was 0.280 for beech and 0.194 for oak. First-order autocorrelation values were similar for both species, amounting to 0.719 for beech and 0.740 for oak. Analysis of basal area increment (BAI) chronologies revealed significant differences in long-term growth patterns between the two species. The oak chronology began earlier and showed a gradual increase in growth from the 18th century to the mid-19th century, after which BAI stabilized at relatively high values (1500–2000 mm2) with moderate interannual variability. In contrast, the beech chronology began later (1768) and exhibited greater temporal variability. Following initially lower values, beech showed a marked increase in growth from the mid-19th century onward, with a continued rise throughout the 20th century. Prior to 1980, both species exhibited statistically significant positive growth trends, slightly more pronounced in oak (β = +6.92 mm2 year−1, p < 0.001) than in beech (β = +1.83 mm2 year−1, p < 0.001). After the 1980s, a divergence in growth trends became evident. In sessile oak, a negative trend was observed (β = −3.29 mm2 year−1), although not statistically significant (p = 0.146). In contrast, beech exhibited a strong and statistically significant increase in growth (β = +18.47 mm2 year−1, p < 0.001), which became even more pronounced after 2000 (β = +19.08 mm2 year−1, p = 0.002). This pattern is reflected in a continuous increase in beech BAI since the 1980s, reaching the highest values in recent decades (>1500 mm2), whereas oak showed a declining trend over the same period (Figure 10a). Comparison of standardized chronologies (z-scores) indicated that both species share similar long-term variability patterns, suggesting a partially common influence of climatic factors on growth. However, the recent divergence—characterized by decreasing growth in oak and increasing growth in beech—indicates species-specific responses to changing environmental conditions (Figure 10b). Overall, both species maintained relatively high BAI values, with beech showing a pronounced increase in recent decades, while oak exhibited a generally stable growth pattern over most of the study period, followed by a decline in the last ~20 years.
Figure 10.
Comparison of basal area increment (BAI) chronologies of oak and beech during the common period. (a) Raw annual BAI values with 10-year moving means and (b) standardized BAI series (z-scores) with 10-year moving means.
4. Discussion
The results of this study indicate that the Muški bunar old-growth forest represents a structurally complex and dynamic forest ecosystem, with changes observed between 1979 and 2021 consistent with general patterns of temperate old-growth forest development [1,3,4,27,28]. The increase in basal area and stand volume, accompanied by relatively minor changes in tree density, suggests a continued biomass accumulation over time. This pattern aligns with the conceptual framework of old-growth forests, where structural development is driven by the interaction of growth, mortality, and disturbance processes rather than by even-aged cohort replacement [6,29]. The recorded deadwood volume (101.36 m3 ha−1) is comparable to values reported for temperate old-growth forests in Europe, where deadwood volumes typically range between approximately 50 and 200 m3 ha−1 [2,3], confirming a high level of structural complexity and advanced developmental stage.
The observed increase in stand volume and basal area further supports the role of old-growth forests as long-term carbon sinks [30]. In this context, the Muški bunar forest corresponds to the pattern of productive yet structurally complex ecosystems [3,31]. Basal area increment (BAI) analysis indicates that both species maintain relatively high growth rates even at advanced ages. However, a clear divergence in growth patterns has emerged in recent decades. Oak shows stagnation and a negative trend after 2000, whereas beech exhibits a continuous increase in growth, particularly since the 1980s. This divergence suggests differences in competitive ability and species-specific responses to environmental change, with beech likely benefiting from its higher plasticity and ability to exploit closed-canopy conditions, while oak appears more sensitive to recent stress factors.
Structural and age-related patterns further reflect differences in species strategies [32]. Beech is well represented across smaller and intermediate diameter and age classes, indicating continuous recruitment, whereas oak is largely confined to older and larger individuals. Similar patterns have been reported in Carpathian old-growth forests, where beech maintains continuous regeneration under small canopy gaps [33,34], while oak is associated with older cohorts and linked to higher-intensity disturbances [8,10,35,36]. The Muški bunar forest confirms these general patterns, but also highlights important deviations in species dynamics. A particularly important finding of this study is the apparent decoupling between disturbance-induced growth response and regeneration success in sessile oak. Although disturbance events were sufficient to stimulate radial growth of existing oak trees, they did not result in successful recruitment, as evidenced by the absence of younger age classes. This pattern is clearly reflected in dendroecological records, where growth release events in oak, particularly during the mid-19th century, were not followed by the establishment of new cohorts.
This decoupling suggests that disturbance alone is not sufficient to ensure oak regeneration. Instead, successful recruitment appears to depend on specific conditions, including sufficient light availability, reduced competition, and suitable microsites. In contrast, beech is capable of regenerating under a wide range of light conditions and can effectively utilize both small- and medium-scale disturbances. These differences highlight fundamental contrasts in life-history strategies and help explain the long-term coexistence patterns observed in mixed beech–oak forests. The observed dynamics may also be influenced by historical land use. Forests in the study area were subject to intensive exploitation during the first half of the 19th century, which likely created canopy openings that promoted the growth of residual oak trees while simultaneously favouring the establishment of shade-tolerant beech. Such legacy effects may contribute to the present-day structure and species composition.
Comparison with Dinaric old-growth forests further emphasizes the specificity of the Muški bunar system. While mixed beech–fir forests maintain structural complexity through continuous regeneration of both species [9,13], oak lacks the ability to persist under prolonged shading. Consequently, management approaches developed for Dinaric systems cannot be directly transferred to beech–oak forests without adaptation [12]. This supports the view that old-growth forests share general structural features but also exhibit strong site- and species-specific dynamics [3]. In the context of climate change, these findings are particularly relevant. Increasing disturbance frequency and intensity are expected across European forests [37], and ecosystem resilience will depend on species-specific responses and their capacity for acclimation [38,39]. The observed divergence between beech and oak suggests that long-term coexistence may be sensitive to changing disturbance regimes and environmental conditions.
Finally, the results should be interpreted in light of certain methodological limitations. Differences in sampling design between the two inventories may influence the estimation of structural attributes, particularly in heterogeneous stands. In addition, dendroecological analysis is constrained by sample size and uncertainties in age estimation. Nevertheless, the consistency among structural, age-related, and dendroecological results supports the robustness of the conclusions.
5. Conclusions
The Muški bunar old-growth forest represents a structurally complex and dynamic mixed stand characterized by pronounced heterogeneity in tree size and age, as well as high growing stock. The results confirm the first hypothesis, as increases in tree dimensions, basal area, and stand volume between 1979 and 2021 indicate continuous natural development and long-term biomass accumulation. The second hypothesis is also supported, as the age structure reflects a multi-cohort dynamic, with continuous regeneration of European beech and the concentration of sessile oak in older age classes.
Stand dynamics are primarily driven by low-intensity disturbances that favour beech, whereas successful regeneration of sessile oak appears to depend on less frequent, high-intensity disturbances and specific microsite conditions. A key finding of this study is the apparent decoupling between growth response and regeneration success in sessile oak, where disturbance-induced growth does not necessarily lead to successful recruitment.
Recent growth trends further indicate a divergence between species, with beech showing increasing growth rates and oak exhibiting stagnation or decline. These results suggest that long-term coexistence in such systems is not based on equilibrium among species, but rather on dynamic interactions shaped by disturbance regimes, species-specific traits, and environmental conditions.
Author Contributions
Conceptualization and methodology, S.M. and L.M.; validation, S.M., D.T., M.O. and I.A.; field investigation, D.T., M.O., K.A. and L.M.; data curation and formal analysis, S.M. and M.O.; writing—original draft preparation, D.T. and M.O.; writing—review and editing, S.M. and I.A.; visualization, D.T. and M.O.; supervision, S.M. and I.A. All authors have read and agreed to the published version of the manuscript.
Funding
This research was funded by the Croatian Science Foundation (HRZZ) project DOK-2025-02 (BIOMONITORING Dendronetwork).
Data Availability Statement
The data presented in this study are available on request from the corresponding author.
Acknowledgments
Authors Stjepan Mikac (SM) and Laura Miketin (LM) acknowledge the support provided by the Croatian Science Foundation (HRZZ).
Conflicts of Interest
The authors declare no conflicts of interest.
References
- Peterken, G.F. Natural Woodland: Ecology and Conservation in Northern Temperate Regions; Cambridge University Press: Cambridge, UK, 1996. [Google Scholar]
- Sabatini, F.M.; Burrascano, S.; Keeton, W.S.; Levers, C.; Lindner, M.; Pötzschner, F.; Verkerk, P.J.; Bauhus, J.; Buchwald, E.; Chaskovsky, O.; et al. Where are Europe’s last primary forests? Divers. Distrib. 2018, 24, 1426–1439. [Google Scholar] [CrossRef] [Scilit]
- Burrascano, S.; Keeton, W.S.; Sabatini, F.M.; Blasi, C. Commonality and variability in the structural attributes of moist temperate old-growth forests: A global review. For. Ecol. Manag. 2013, 291, 458–479. [Google Scholar] [CrossRef] [Scilit]
- Franklin, J.F.; Spies, T.A.; Van Pelt, R.; Carey, A.B.; Thornburgh, D.A.; Berg, D.R.; Lindenmayer, D.B.; Harmon, M.E.; Keeton, W.S.; Shaw, D.C.; et al. Disturbances and structural development of natural forest ecosystems with silvicultural implications, using Douglas-fir forests as an example. For. Ecol. Manag. 2002, 155, 399–423. [Google Scholar] [CrossRef] [Scilit]
- Nagel, T.A.; Svoboda, M.; Kobal, M. Disturbance, life history traits, and dynamics in an old-growth forest landscape of southeastern Europe. Ecol. Appl. 2014, 24, 663–679. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pickett, S.T.A.; White, P.S. The Ecology of Natural Disturbance and Patch Dynamics; Academic Press: Orlando, FL, USA, 1985. [Google Scholar]
- Nagel, T.A.; Svoboda, M.; Diaci, J. Regeneration patterns after intermediate wind disturbance in an old-growth Fagus–Abies forest in southeastern Slovenia. For. Ecol. Manag. 2006, 226, 268–278. [Google Scholar] [CrossRef] [Scilit]
- Petritan, A.M.; Nuske, R.S.; Petritan, I.C.; Tudose, N.C. Gap disturbance patterns in an old-growth sessile oak (Quercus petraea L.)—European beech (Fagus sylvatica L.) forest remnant in the Carpathian Mountains, Romania. For. Ecol. Manag. 2013, 308, 67–75. [Google Scholar] [CrossRef] [Scilit]
- Diaci, J.; Rozenbergar, D.; Anić, I.; Mikac, S.; Saniga, M.; Kucbel, S.; Visnjic, C.; Ballian, D. Structural dynamics and synchronous silver fir decline in mixed old-growth mountain forests in Eastern and Southeastern Europe. Forestry 2011, 84, 479–491. [Google Scholar] [CrossRef] [Scilit]
- Petritan, I.C.; Marzano, R.; Petritan, A.M.; Lingua, E. Overstory succession in a mixed Quercus petraea—Fagus sylvatica old-growth forest revealed through the spatial pattern of competition and mortality. For. Ecol. Manag. 2014, 326, 132–141. [Google Scholar] [CrossRef] [Scilit]
- Bauhus, J.; Puettmann, K.J.; Messier, C. Silviculture for old-growth attributes. For. Ecol. Manag. 2009, 258, 525–537. [Google Scholar] [CrossRef] [Scilit]
- O’Hara, K.L. Multiaged Silviculture: Managing for Complex Forest Stand Structures; Oxford University Press: Oxford, UK, 2014. [Google Scholar]
- Keren, S.; Diaci, J.; Motta, R.; Govedar, Z. Stand structural complexity of mixed old-growth and adjacent selection forests in the Dinaric Mountains of Bosnia and Herzegovina. For. Ecol. Manag. 2017, 400, 531–541. [Google Scholar] [CrossRef] [Scilit]
- Petritan, A.M.; Bouriaud, O.; Frank, D.C.; Petritan, I.C. Dendroecological reconstruction of disturbance history of an old-growth mixed sessile oak–beech forest. J. Veg. Sci. 2016, 27, 1125–1135. [Google Scholar] [CrossRef] [Scilit]
- Vukelić, J.; Baričević, D.; Šapić, I. Submontansko-subpanonske bukove šume sjeverne Hrvatske. Šumarski List 2012, 136, 445–459. Available online: https://hrcak.srce.hr/91427 (accessed on 6 April 2026).
- Matić, S.; Prpić, B.; Rauš, Đ.; Vranković, A.; Seletković, Z. Ekološko-uzgojne osobine specijalnih rezervata šumske vegetacije Prašnik i Muški bunar u Slavoniji. In Drugi Kongres Ekologa Jugoslavije; Rauš, Đ., Ed.; Savez Društava Ekologa Jugoslavije: Zagreb, Croatia, 1979; pp. 767–823. [Google Scholar]
- Phipps, R.L. Collecting, Preparing, Crossdating, and Measuring Tree Increment Cores; U.S. Geological Survey: Reston, VA, USA, 1985.
- Levanič, T. ATRICS—A new system for image acquisition in dendrochronology. Tree-Ring Res. 2008, 63, 117–122. [Google Scholar] [CrossRef] [Scilit]
- Baillie, M.G.L.; Pilcher, J.R. A simple cross-dating program for tree-ring research. Tree-Ring Bull. 1973, 33, 7–14. Available online: http://hdl.handle.net/10150/260029 (accessed on 8 April 2026).
- Schweingruber, F.H. Tree Rings: Basics and Applications of Dendrochronology; Kluwer Academic Publishers: Dordrecht, The Netherlands, 1988. [Google Scholar]
- Holmes, R.L. Computer-assisted quality control in tree-ring dating and measurement. Tree-Ring Bull. 1983, 43, 69–78. [Google Scholar]
- Nowacki, G.J.; Abrams, M.D. Radial-growth averaging criteria for reconstructing disturbance histories from presettlement-origin oaks. Ecol. Monogr. 1997, 67, 225–249. [Google Scholar] [CrossRef] [Scilit]
- Altman, J.; Fibich, P.; Dolezal, J.; Aakala, T. TRADER: A package for tree ring analysis of disturbance events in R. Dendrochronologia 2014, 32, 107–112. [Google Scholar] [CrossRef] [Scilit]
- Bunn, A.G. A Dendrochronology Program Library in R (dplR). Dendrochronologia 2008, 26, 115–124. [Google Scholar] [CrossRef] [Scilit]
- Silva, C.A.; Valbuena, R.; Pinagé, E.R.; Mohan, M.; de Almeida, D.R.A.; Broadbent, E.N.; Mohd Jaafar, W.S.W.; de Almeida Papa, D.; Cardil, A.; Klauberg, C. ForestGapR: An R Package for Forest Gap Analysis from Canopy Height Models. Methods Ecol. Evol. 2019, 10, 1347–1356. [Google Scholar] [CrossRef] [Scilit]
- Solano, F.; Modica, G.; Praticò, S.; Box, O.F.; Piovesan, G. Unveiling the Complex Canopy Spatial Structure of a Mediterranean Old-Growth Beech (Fagus sylvatica L.) Forest from UAV Observations. Ecol. Indic. 2022, 138, 108807. [Google Scholar] [CrossRef] [Scilit]
- Mölder, A.; Bernhardt-Römermann, M.; Schmidt, W. Herb-layer diversity in deciduous forests: Raised by tree richness or beaten by beech? For. Ecol. Manag. 2008, 256, 272–281. [Google Scholar] [CrossRef] [Scilit]
- Johnson, P.S.; Shifley, S.R.; Rogers, R. The Ecology and Silviculture of Oaks, 2nd ed.; CABI: Wallingford, UK, 2009. [Google Scholar]
- Emborg, J.; Christensen, M.; Heilmann-Clausen, J. The structural dynamics of a near-natural temperate deciduous forest. For. Ecol. Manag. 2000, 126, 173–189. [Google Scholar] [CrossRef] [Scilit]
- Martin-Benito, D.; Pederson, N.; Férriz, M.; Gea-Izquierdo, G. Old forests and old carbon: A case study on the stand dynamics and longevity of aboveground carbon. Sci. Total Environ. 2021, 765, 142737. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pretzsch, H. Forest Dynamics, Growth and Yield; Springer: Berlin, Germany, 2009. [Google Scholar] [CrossRef] [Scilit]
- Westphal, C.; Tremer, N.; von Oheimb, G.; Hansen, J.; von Gadow, K.; Härdtle, W. Is the reverse J-shaped diameter distribution universally applicable in European virgin beech forests? For. Ecol. Manag. 2006, 223, 75–83. [Google Scholar] [CrossRef] [Scilit]
- Jaloviar, P.; Sedmáková, D.; Pittner, J.; Dankova, L.J.; Kucbel, S.; Sedmak, R.; Saniga, M. Gap structure and regeneration in the mixed old-growth forests of National Nature Reserve Sitno, Slovakia. Forests 2020, 11, 81. [Google Scholar] [CrossRef] [Scilit]
- Petritan, A.M.; Toiu, F.L.; Tudose, N.C.; Petritan, I.C. Patterns of sessile oak regeneration and its main drivers in an old-growth sessile oak–European beech forest. Eur. J. For. Res. 2025, 144, 1395–1408. [Google Scholar] [CrossRef] [Scilit]
- Ellenberg, H.; Leuschner, C. Vegetation Ecology of Central Europe, 6th ed.; Springer: Cham, Switzerland, 2017. [Google Scholar]
- Petritan, A.M.; Biris, I.A.; Merce, O.; Turcu, D.O.; Petritan, I.C. Structure and diversity of a natural temperate sessile oak (Quercus petraea L.)—European beech (Fagus sylvatica L.) forest. For. Ecol. Manag. 2012, 280, 140–149. [Google Scholar] [CrossRef] [Scilit]
- Seidl, R.; Thom, D.; Kautz, M.; Martin-Benito, D.; Petloniemi, M.; Vacchiano, G.; Wild, J.; Ascoli, D.; Petr, M.; Honkaniemi, J.; et al. Forest disturbances under climate change. Nat. Clim. Chang. 2017, 7, 395–402. [Google Scholar] [CrossRef] [Scilit]
- Mori, A.S.; Furukawa, T.; Sasaki, T. Response diversity determines the resilience of ecosystems to environmental change. Biol. Rev. 2013, 88, 349–364. [Google Scholar] [CrossRef] [Scilit]
- Pretzsch, H.; Schütze, G.; Uhl, E. Resistance of European tree species to drought stress in mixed versus pure forests: Evidence of stress release by inter-specific facilitation. Plant Biol. 2013, 15, 483–495. [Google Scholar] [CrossRef] [Scilit]
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.