


Abstract
The diversity of macrofungi has been closely associated with forest diversity and stability. However, such a correlation has not been established for the forests of the Ningxia Autonomous Region due to the lack of systematic data on its macrofungal diversity. Therefore, for the present study, we collected 3130 macrofungal specimens from the forests of the Helan Mts., Luo Mts., and Liupan Mts. in Ningxia and assessed them using morphological and molecular approaches. We identified 468 species belonging to 157 genera, 72 families, 18 orders, 11 classes, and 2 phyla. Among them, 31 species were ascomycetes, and 437 species were basidiomycetes. Tricholomataceae, with 96 species of 22 genera, was the most species-rich family, and Inocybe was the most species-rich genus (6.2%). The Jaccard similarity index measurement revealed the highest similarity in macrofungal species (16.15%) between the Helan and Liupan Mountains and the lowest (7.72%) between the Luo and Liupan Mountains. Further analyses of the macrofungal population of Ningxia showed that 206 species possess considerable potential for utilization, including 172 edible, 70 medicinal, and 36 edible–medicinal ones. Meanwhile, 54 species were identified as being poisonous. In these forests, saprophytic fungi were the most abundant, with 318 species (67.95%), followed by symbiotic fungi (31.62%) and parasitic fungi (0.04%). Grouping based on the geographical distribution indicated that the fungi of Ningxia are composed mainly of the cosmopolitan and north temperate types. These observations unveil the diversity and community structure of macrofungi in Ningxia forests.
1. Introduction
Macrofungi are fungal species that produce large basidiocarps or ascocarps and are visible to the naked eye. These fungi belong to two main phyla, the Basidiomycota and the Ascomycota. About 160–170 thousand macrofungal species are found worldwide, of which only 16 thousand (10%) have been characterized [1]. Macrofungi are distributed in diverse habitats, such as forests, grasslands, deserts, and oceans, with the highest species diversity detected in forest ecosystems [2,3,4]. China’s vast forest cover provides a favorable environment for the survival and expansion of macrofungi. A total of 4250 species of macrofungi had been discovered in the forests of China by 2021 [5].
The diversity of macrofungi is a crucial factor that regulates and improves forest ecosystem functions. As a nutrient-cycling component, the saprophytic and some pathogenetic macrofungi help degrade forest litter and release nutrients [6,7]. Consequently, they influence forest regeneration by regulating the efficiency of nutrient utilization by different plant species [8]. Many macrofungi establish symbiotic relationships with plants, enhance the absorption of water and nutrients, increase the ability of carbon synthesis, and improve resistance against stress and the plants’ survival rates [9]. These macrofungi, called mycorrhizal fungi, positively influence plant traits and regulate plant interactions with soil, altering various ecosystem processes [10]. Mycorrhizal fungi also influence plant community dynamics in forests by fixing nitrogen from the atmosphere and protecting plants from pathogen attacks [11,12]. All these functions of macrofungi are necessary for maintaining forest biodiversity and stability.
Edible and medicinal mushrooms are macrofungi with considerable economic value. More than 2200 species of macrofungi found worldwide are edible and/or medicinal [13]. China has remarkable microfungal diversity, with around 1020 edible and/or medicinal species making up approximately 50% of the world’s resources [14]. Edible mushrooms are considered top-tier food materials due to their high protein, low sugar, low fat, and low cholesterol levels. Moreover, the polysaccharides in mushrooms directly interact with the cell membrane receptors of humans, resulting in extensive pharmacological activity without any side effects [15]. Mushroom foraging is becoming increasingly popular in many countries, as it provides food and income for local people [16,17,18]. In China, the mushroom industry is the fifth largest agricultural industry, producing more than 70% of the mushroom yield from the wild [19]. As a major source of mushroom foraging, wild resources of macrofungi found in forests deserve more attention.
The Ningxia Autonomous Region has almost 5.13 × 10⁵ hectares of forest land, which accounts for 9.88% of the total forest cover in China. This region, located in the northwest area of China, lies in the upper reaches of the Yellow River and the transitional zone between the Loess Plateau and the Inner Mongolian Plateau. However, currently, there are no systematic data available on the diversity of macrofungi in the forests of the Ningxia Autonomous Region, except for a few sporadic reports [20,21,22,23].
Therefore, the present study investigated the diversity of macrofungi in the forests of the Ningxia Autonomous Region. We collected multiple macrofungal samples from the forests of the Ningxia Autonomous Region from 2018 to 2023 and analyzed them using morphological and molecular biology methods. Furthermore, we analyzed their macrospecies composition, economic value, and nutritional type.
2. Materials and Methods
2.1. Sample Plot
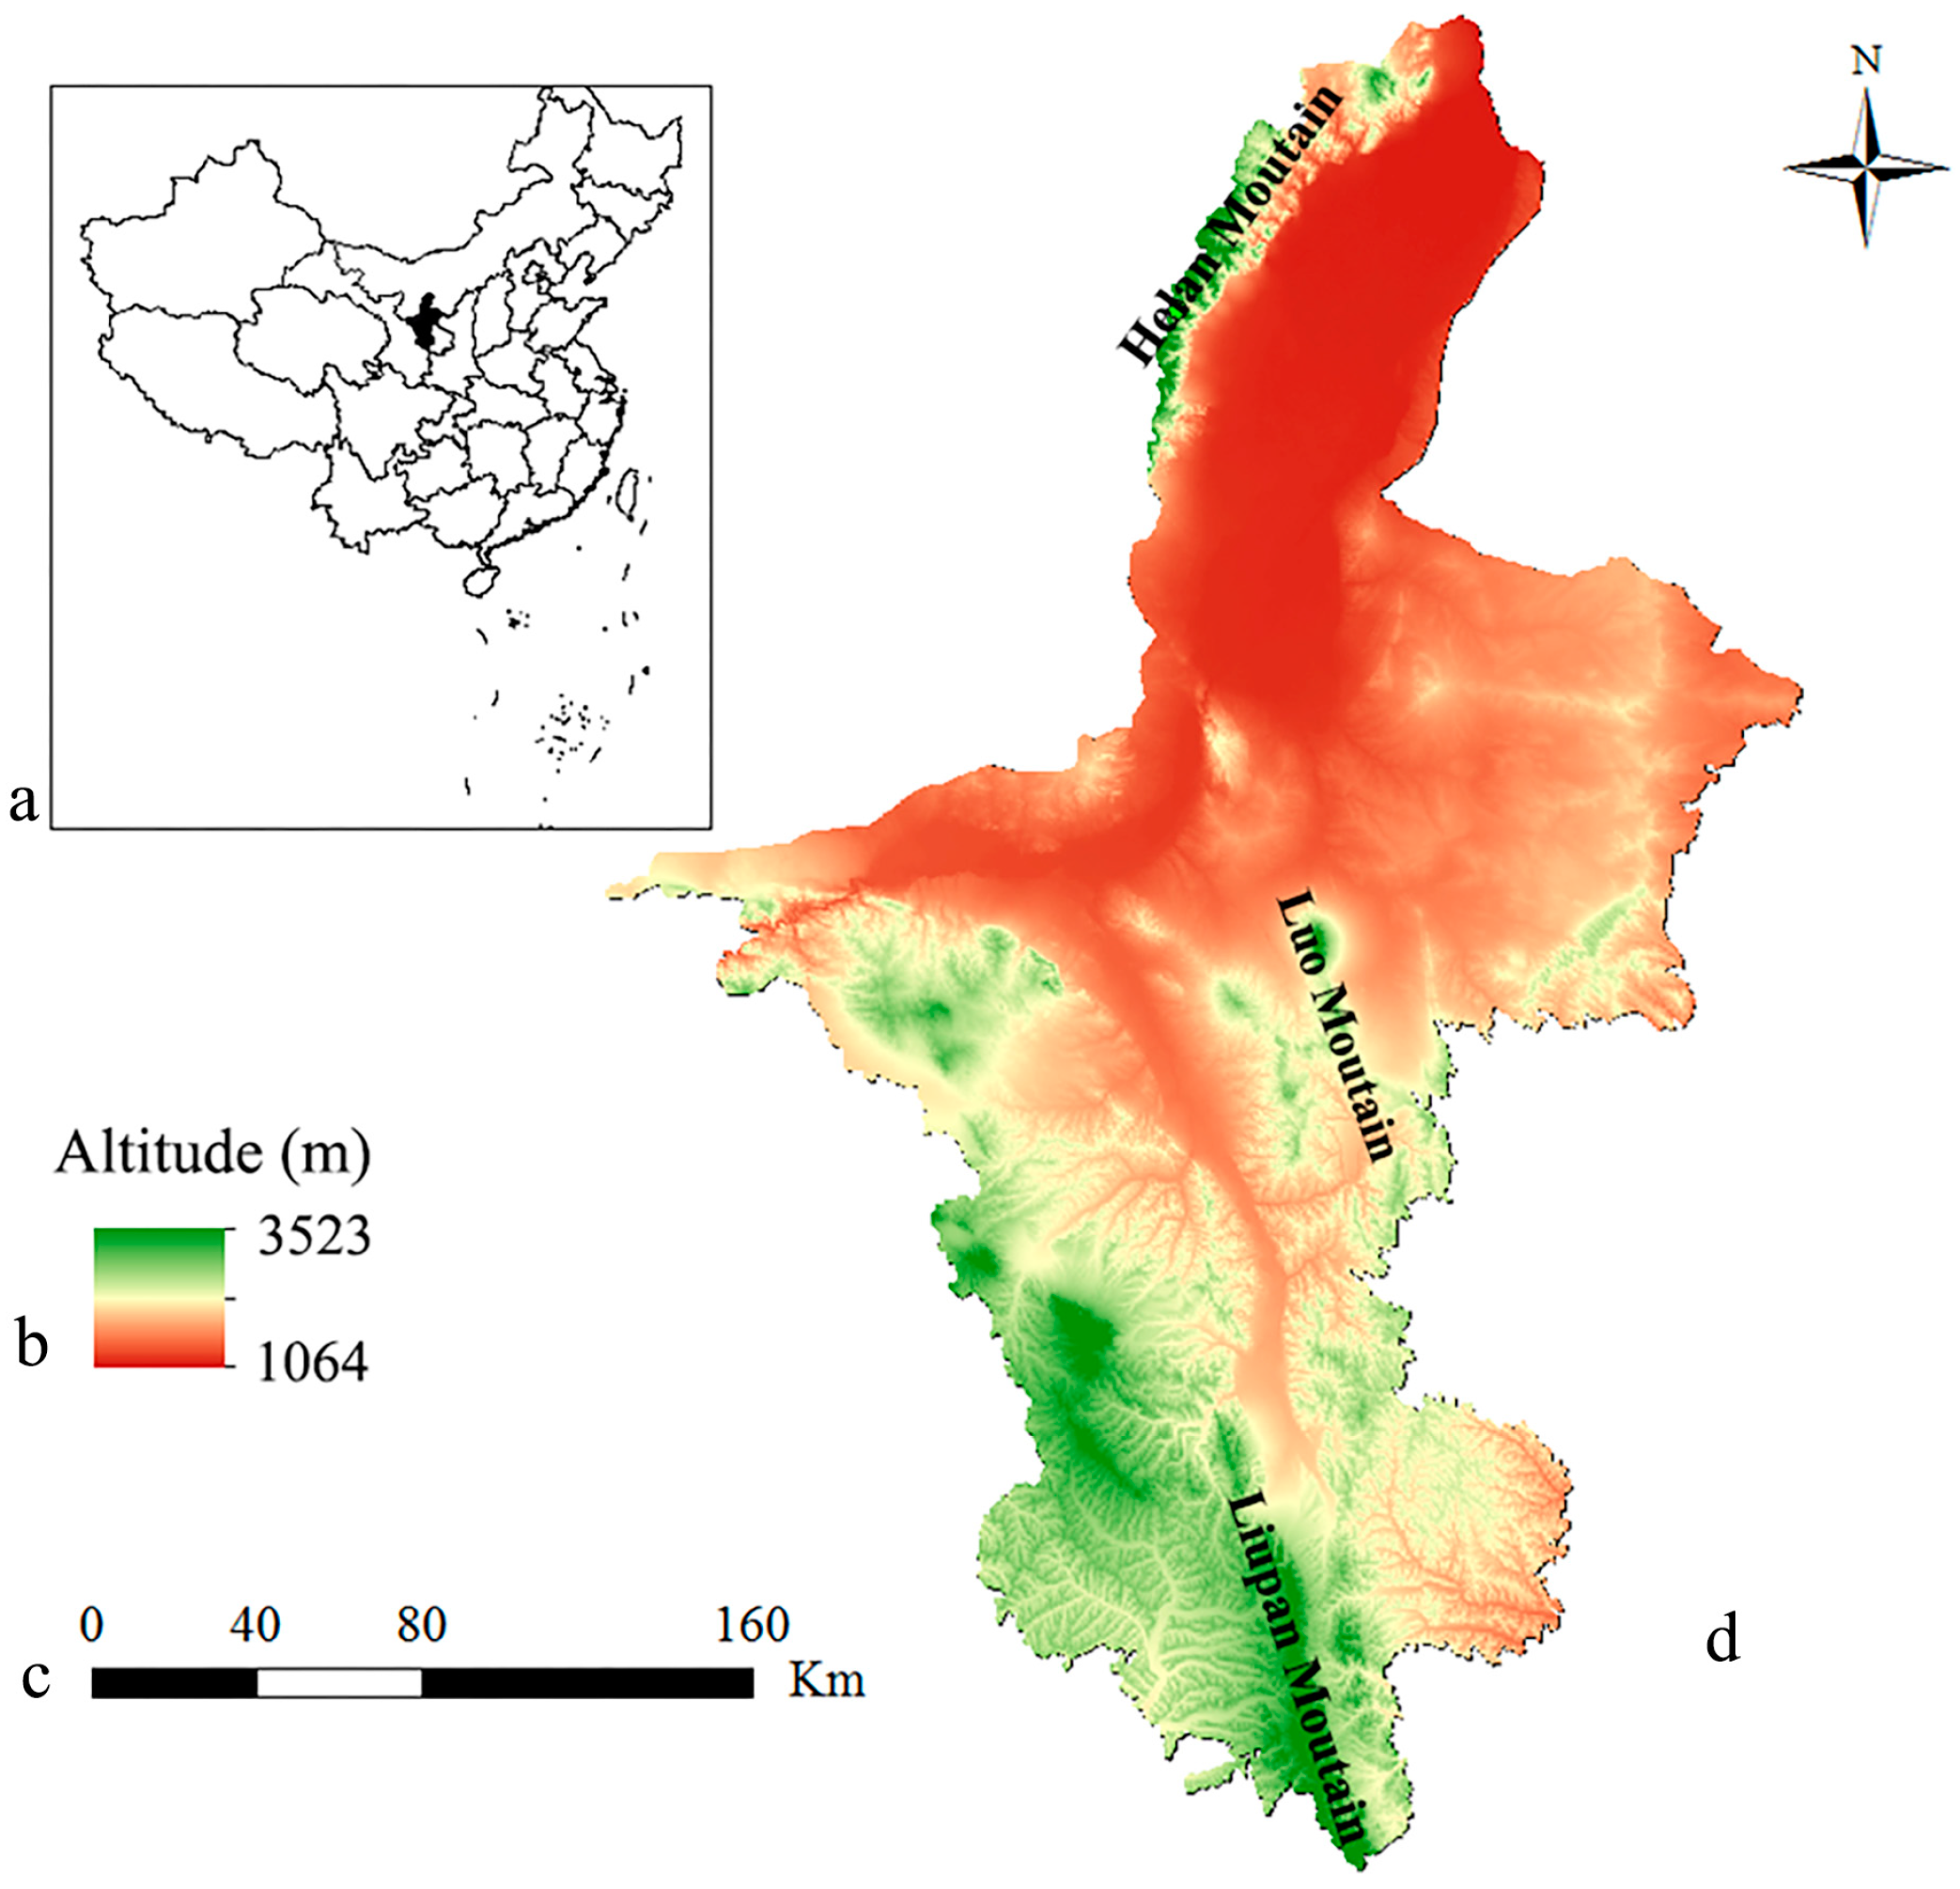
The present study analyzed macrofungi from three major forest zones in the Ningxia Autonomous Region of China, including the Helan Mountains (2.8 × 10⁴ ha), Luo Mountains (6.4 × 10³ ha), and Liupan Mountains (5.14 × 10⁴ ha) (Figure 1). The Helan Mountains are located in the north of the Ningxia Autonomous Region at a junction of temperate grassland and desert and have primarily coniferous forest vegetation (1900–3000 m). The average temperature is 22 °C in summer and −10 °C in winter, with an annual precipitation of about 430 mm. Picea crassifolia, Pinus tabuliformis, and Populus davidiana are the major constructive species of the forest in the Helan Mountains, with the cinnamon soil type [24]. The Luo Mountains are an ecological barrier and water conservation area located in the central arid region of the Ningxia Autonomous Region. The average temperature is 21 °C in summer and −7 °C in winter, with an annual precipitation of about 296 mm. The dominant vegetation type is constructive species, such as Picea crassifolia and Pinus tabuliformis, with the sierozem soil type [25]. The Liupan Mountains are located in the southern part of the Ningxia Autonomous Region and provide a unique natural defense for the Loess Plateau. The average temperature is 18 °C in summer and −7 °C in winter, with an annual precipitation of about 676 mm. The Liupan Mountains are covered by temperate coniferous forests comprising coniferous species, such as Larix principis-rupprechtii and Pinus sylvestris var. mongolica, and secondary deciduous broad-leaved mixed forests with species such as Quercus wutaishanica, Betula platyphlla, and Populus davidiana, with the grey–cinnamon soil type [26].
Figure 1.
The location of the Ningxia Province in China (a) and forest distribution in Ningxia Province (d). (b) Colors indicate the altitude of different sites in the Ningxia Province. (c) Geographic scale.
Based on forest topography, vegetation type, and transport accessibility, macrofungal specimens were collected from 14 sample plots (Table 1). Four sample plots were in the Helan Mountains (Yingtao Valley, Tu Er Keng, Tou Dao Song, and Da Shui Gou), four were in the Luo Mountains (Da Luo Shan, Xiao Luo Shan, Lu Hua Tai Gou, and Hao Han Feng), and six were in the Liupan Mountains (Wang Hua Nan, Da Dao Gou, Xiao Dao Gou, Xiao Nan Chuan, Ye He Gu, and the botanical garden).
Table 1.
Information of sample plots.
2.2. Collection of Macrofungal Specimens
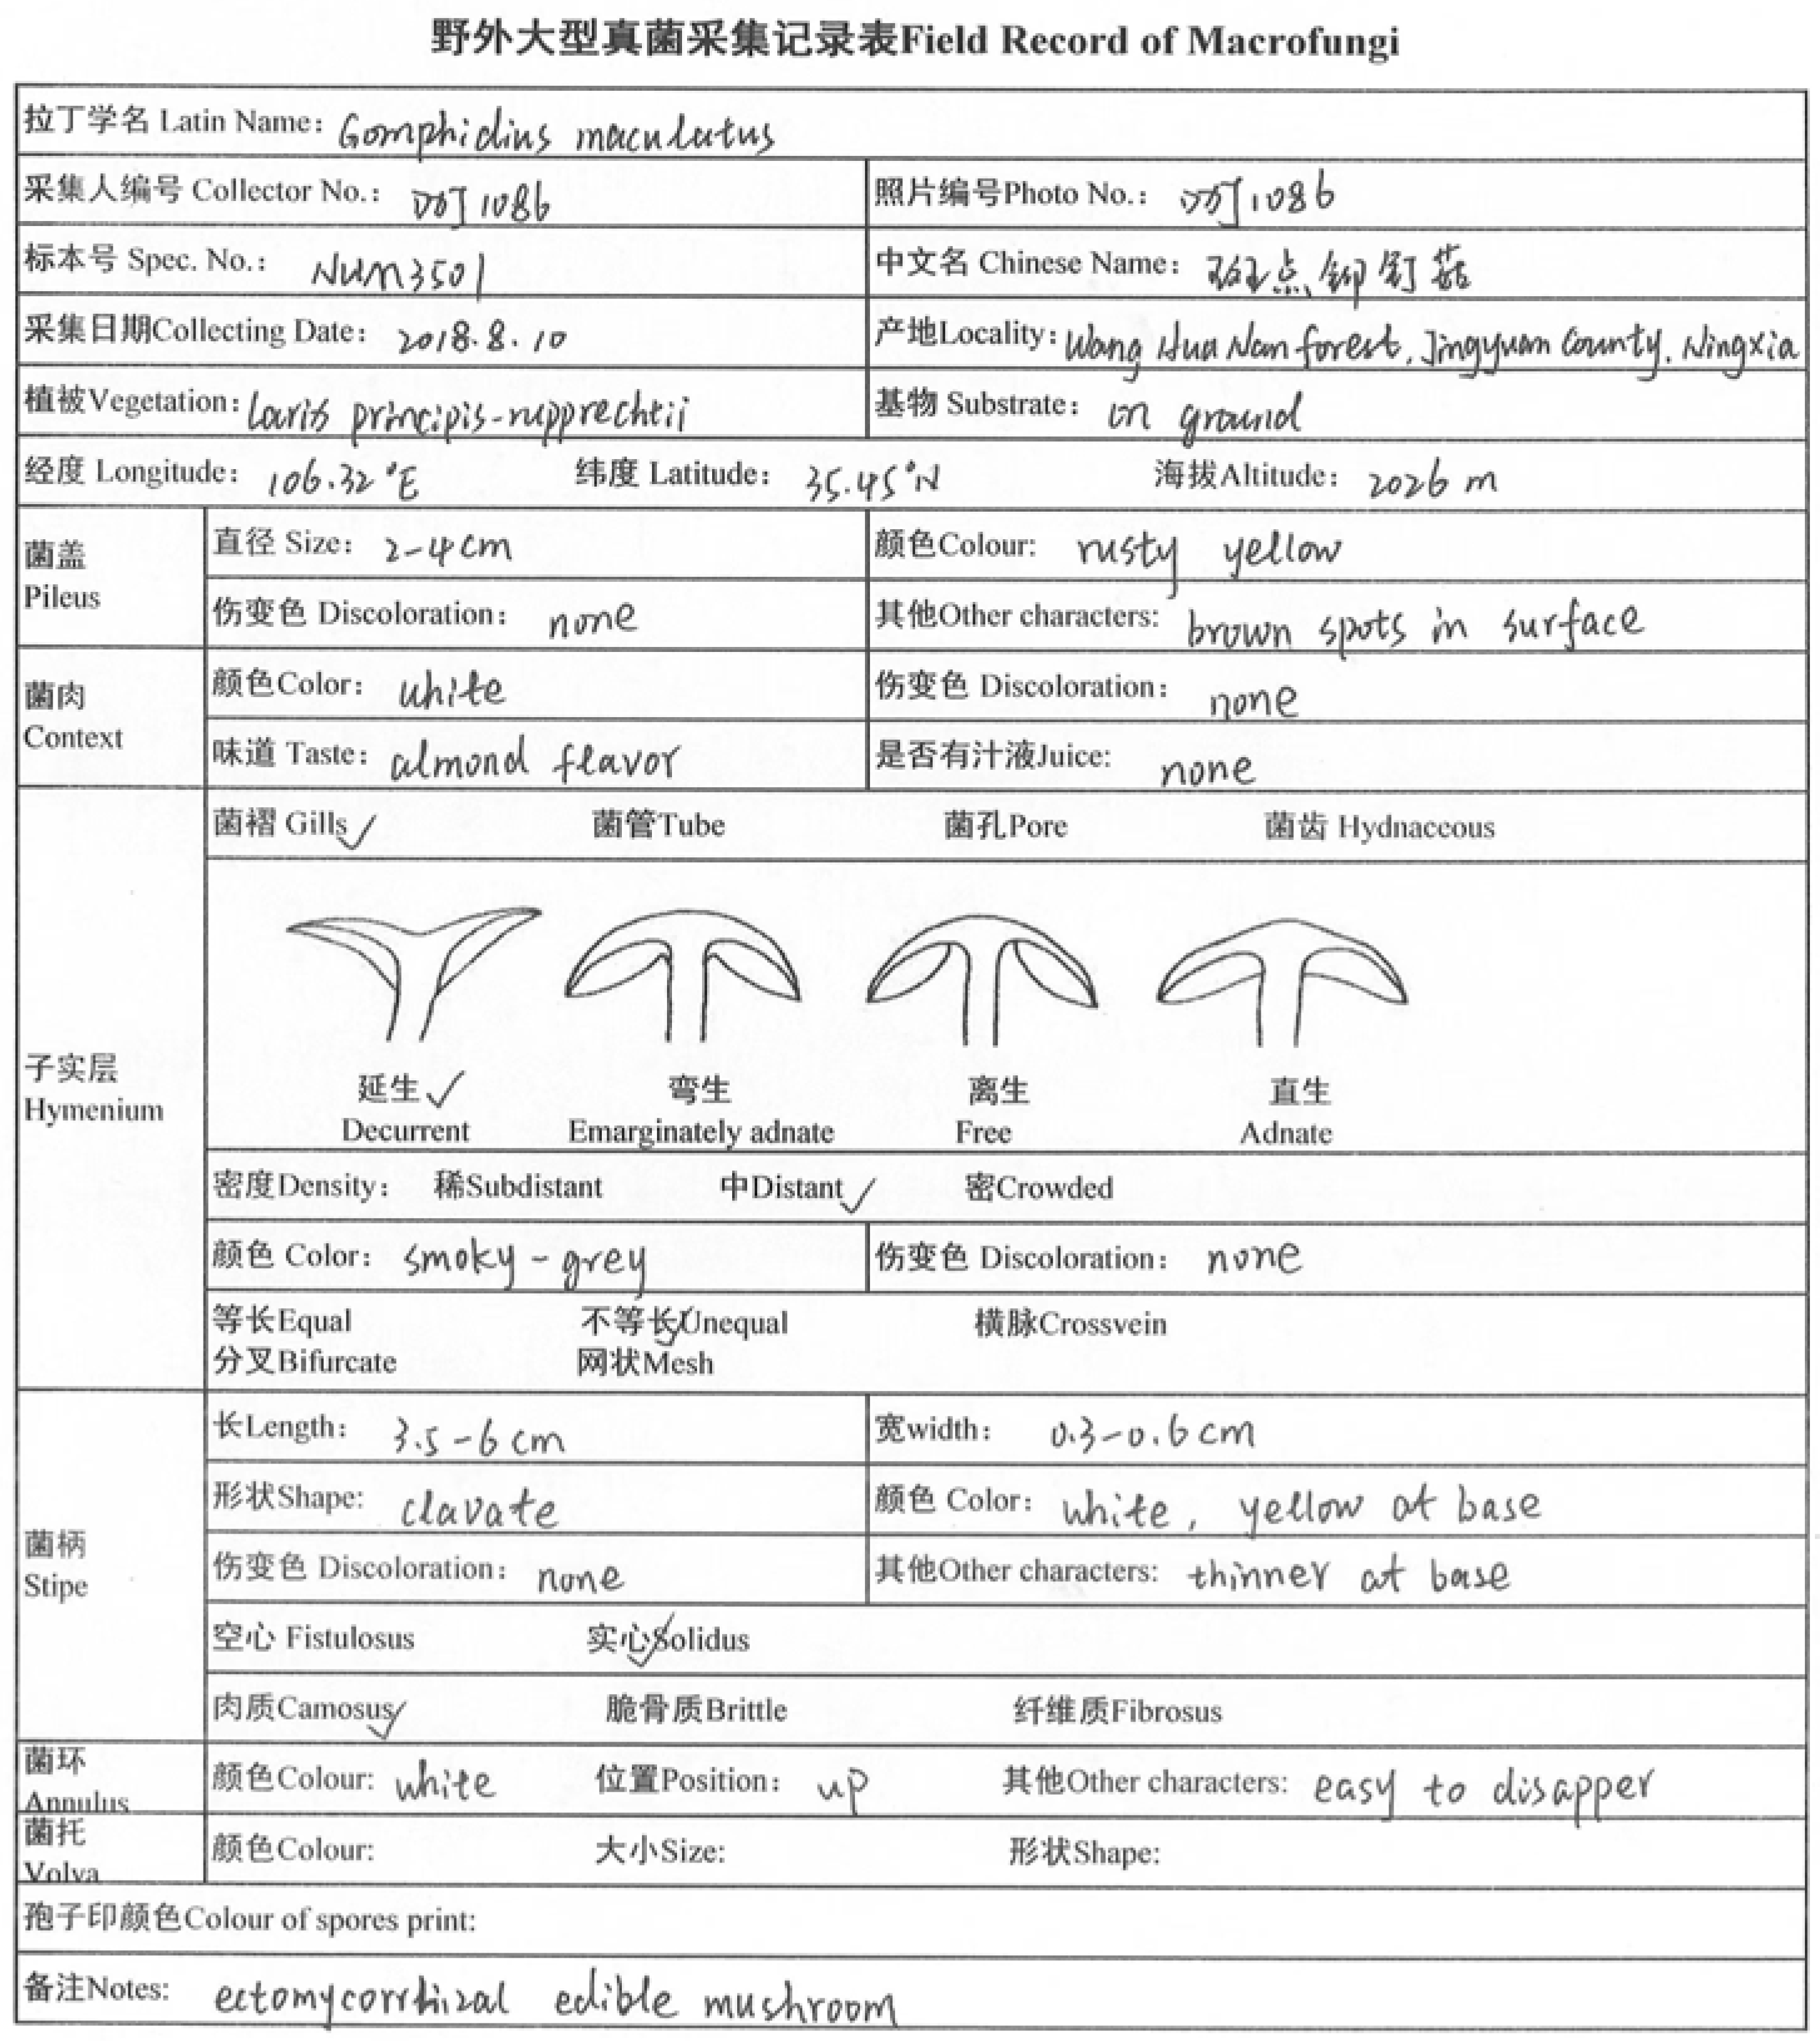
All basidiocarps and ascocarps from each sample plot were collected following a random stepping method. From 2018 to 2023, collections were conducted once a month at all sample plots from June to September, with each collection lasting for one day for plots with a size of less than 4.0 × 10⁴ m2 and two days for each bigger plot. Images of the basidiocarps and ascocarps were captured immediately after collection, and the sampling site and the integral details, including the pileus and hymenium of these freshly collected basidiocarps and ascocarps, were recorded (Figure 2). The basidiocarps and ascocarps were then dried in an oven at 55 °C and stored at 10–15 °C in a specimen bag.
Figure 2.
An example of the field records of a collected specimen.
2.3. Morphological Analysis
All collected specimens were deposited in the herbarium of North Minzu University (NMU). The macro-morphological details of the basidiocarps and ascocarps, including the color, shape, size, and appendages in the surfaces of the cap, stipe, and hymenium (lamellated, poroid, hydnoid, and corticioid), were analyzed and recorded based on the field notes (Figure 2). Similarly, the micro-morphological details of the epidermis, hymenium, spores, and mycelia were observed in a 5% KOH solution in dry specimens using a Nikon E400 biological microscope [27,28,29]. The morphological identification process was mostly based on significant references [30,31,32,33,34,35,36,37,38,39]. The identified species names were verified in the Index Fungorum (www.indexfungorum.org) or MycoBank (www.mycobank.org) accessed on 10 November 2024 to ensure the accuracy of the species names.
2.4. Molecular Analysis
When we were unable to identify species using morphological approaches, molecular analysis was used to assist in their identification. The total DNA was isolated from the macrofungal dried specimens using a rapid fungal genomic DNA isolation kit (Sangon Biotech Co., Ltd., Shanghai, China). Polymerase chain reaction (PCR) was performed with the obtained DNA and the ITS1F [40] and ITS4 [41] primers according to the method by Liu et al. (2023) [42] to amplify the fungal internal transcribed spacer (ITS). The amplicons were sequenced at Sangon Biotech Co., Ltd. (Shanghai, China). The ITS sequences were assembled and quality-checked using Contig Express (v3.0.0) software and then submitted to the NCBI or UNITE databases for BLAST. High-homology sequences were selected, and then multi-sequence alignment construction was performed using BioEdit (7.2.5) and MAFFT-7.505 (https://mafft.cbrc.jp/alignment/software) software. A phylogenetic tree was constructed using the maximum likelihood method (ML) with RAxML (Windows Executables v8.2.10) software, and it was processed using FigTree (v1.4.0) software. Finally, species identification was conducted based on the morphological characteristics of the specimens and the sequence alignment results [43].
2.5. Analysis of Species Composition
The species were counted and sorted based on family and genus. Families with ≥10 species and genera with ≥5 species were identified as dominant [44].
The Jaccard similarity index (Jsim) was calculated using the following equation to assess the differences in the macrofungal species compositions among the Helan, Luo, and Liupan Mountains [45]:
Jsim = c/(a + b − c) × 100%, where Jsim is the Jaccard similarity index, a and b are the numbers of species in sample plots 1 and 2, and c is the number of species shared among plots 1 and 2. A higher Jaccard similarity index means greater fungal similarity and closer fungal relationships among the forests.
Based on published data, the identified macrofungal species were categorized as edible, medicinal, edible–medicinal, or poisonous [14]. Similarly, based on the published details on the trophic type, the macrofungi were grouped as saprophytic, symbiotic, or parasitic [30].
2.6. Analysis of Funga
Funga are related to fungal flora. This study defined the funga based on previous data [46,47,48,49].
3. Results
3.1. Macrofungal Composition in the Forests of the Ningxia Autonomous Region
We collected 3130 macrofungal specimens, including 1236 from the Helan Mountains, 329 from the Luo Mountains, and 1565 from the Liupan Mountains. The number of specimens corresponded to the size of the forest in each mountain. From these specimens, 468 species were identified, of which 119 species were identified by molecular method, belonging to 157 genera, 72 families, 18 orders, 11 classes, and 2 phyla (Table 2). Among them, 31 species belonging to 7 genera, 11 families, 6 orders, and 4 classes were ascomycetes, and 437 species belonging to 150 genera, 61 families, 12 orders, and 7 classes were basidiomycetes (Table 2). These initial observations indicated an abundance of macrofungi in the forests of the Ningxia Autonomous Region. Specifically, basidiomycetes dominated these forests (Table 2).
Table 2.
Composition of macrofungi in the forests of the Ningxia Autonomous Region.
3.2. Dominant Macrofungal Families and Genera in the Forests of the Ningxia Autonomous Region
3.2.1. Dominant Families
In-depth analysis revealed divergence in the dominant families among the forests of the Ningxia Autonomous Region (Table 3). The Liupan Mountains had nine dominant families, in which Tricholomataceae was the most species-rich one, with 29 species of 10 genera (11.46%), followed by Strophariaceae, with 22 species of 5 genera (8.7%), and Psathyrellaceae, with 18 species of 5 genera (7.11%). Similarly, four families dominated the forests of the Helan Mountains, where Tricholomataceae was the most species-rich, with 55 species of 16 genera (23.31%). However, only two families dominated the Luo Mountains (Tricholomataceae and Inocybaceae, with 12 species each).
Table 3.
Differences in the dominant macrofungal families (≥10 species) among the forests of the Ningxia Autonomous Region.
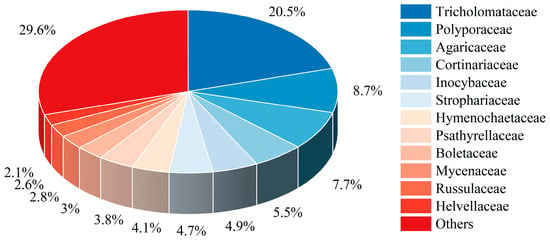
Combining the observations from all the regions, 12 families (≥10) encompassing 330 species of 86 genera (70.51% of the total species) were found to be dominant in the forests of the Ningxia Autonomous Region. The most species-rich family was Tricholomataceae (96 species in 22 genera; 20.51% of the total species), which was followed by Polyporaceae (41 species; 8.7%) and Agaricaceae (36 species; 7.69%) (Figure 3).
Figure 3.
Dominant macrofungal families (≥10 species) in the forests of the Ningxia Autonomous Region.
3.2.2. Dominant Genera
The dominant genera also differed among the forests of the Ningxia Autonomous Region (Table 4). A total of 18 dominant genera with 119 species (44.24%) were identified in the Liupan Mountains, in which the most species-rich genus was Mycena (13 species; 5.14%), followed by Inocybe (11 species; 4.35%) and Helvella (8 species; 3.16%). Meanwhile, 11 genera with 100 species (42.37%) dominated in the Helan Mountains, in which the most species-rich genus was Cortinarius (16 species; 6.8%), followed by Clitocybe (14 species; 5.93%) and Tricholoma (12 species; 5.08%) and Agaricus (12 species; 5.1%). Inocybe, including 12 species (14.63%), was the only dominant genus in the Luo Mountains.
Table 4.
Dominant macrofungal genera (≥5 species) among the forests of the Ningxia Autonomous Region.
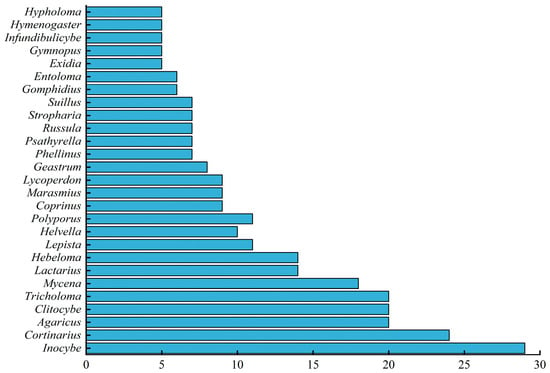
Combining the data from all regions analyzed in this study, 27 genera with 298 species were identified as the dominant ones in the Ningxia macrofungi; these species accounted for 63.68% of the total species (Figure 4). The most species-rich genus was Inocybe, with 29 species (6.2% of the total species), followed by Cortinarius, with 24 species (5.13%).
Figure 4.
Dominant macrofungal genera (≥5 species) in the forests of the Ningxia Autonomous Region. The ordinate shows the dominant genera, and the abscissa indicates the number of species in each genus.
3.3. Species Similarity Among the Forests of the Ningxia Autonomous Region
The forest macrofungal species of the Helan Mountains, Luo Mountains, and Liupan Mountains were compared based on the Jaccard similarity index to assess their differences in composition. The Jaccard similarity index was the highest (16.15%) between the Helan and Liupan Mountains, with the maximum shared species and the highest similarity in species composition. Meanwhile, the index was the lowest (7.72%) between the Liupan and Luo Mountains, with the fewest shared species and the lowest similarity in species composition (Table 5).
Table 5.
Species similarity among the forests of Ningxia Autonomous Region (%).
3.4. Classification of Macrofungi Based on Function and Trophic Type in the Forests of the Ningxia Autonomous Region
Analysis of the macrofungal species identified in the Ningxia Autonomous Region revealed that 207 species of 10 genera, 8 families, 3 orders, and 2 classes possessed potential values; these species were primarily edible and medicinal mushrooms. The analysis identified 173 edible species (36.97% of total species), 70 medicinal species (14.96%), and 36 edible–medicinal species (7.69%) (Table 6). In addition, 54 poisonous species were also identified from the forests of the Ningxia Autonomous Region (11.54%).
Table 6.
Macrofungal functions and trophic types in the forests of Ningxia Autonomous Region.
Further grouping based on the trophic type revealed that the Ningxia Autonomous Region had mostly saprophytic macrofungi, with 333 species (71.15% of the total species), symbiotic fungi (133 species; 28.42%), and parasitic fungi (2 species; Cordyceps sp. and Cordyceps ningxiaensis) (Table 6). Among the 253 species distributed in the Liupan Mountains, 191 were saprophytic (75.49%), 60 were symbiotic (23.72%), and 2 were parasitic (0.8%). Among the 236 species of the Helan Mountains, 183 were saprophytic (77.54%), and 53 were symbiotic (22.46%). Among the 82 species of the Luo Mountains, 52 were saprophytic (63.41%), and 30 were symbiotic (36.59%).
3.5. Analysis of the Funga of the Forests of the Ningxia Autonomous Region
3.5.1. Families in the Funga
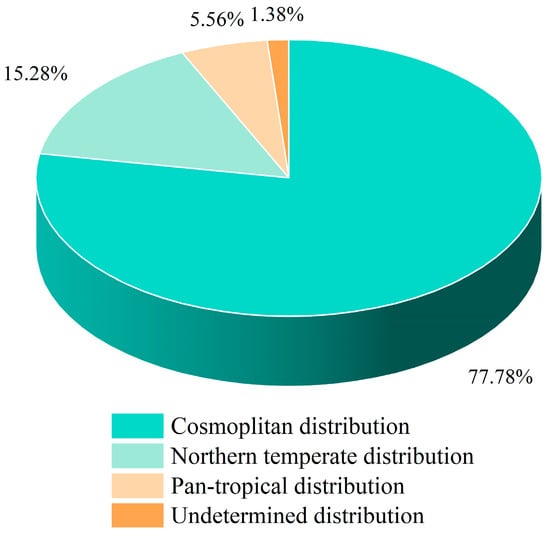
Finally, analysis of the geographical distribution pattern showed that macrofungi with cosmopolitan distribution dominated the forests of the Ningxia Autonomous Region (77.78% of total families) (Figure 5). Cudoniaceae, Lyophyllaceae, Hygrophoraceae, Helvellaceae, Tuberaceae, Sarcosomataceae, Exidiaceae, Fistulinaceae, Bolbitiaceae, Coniophoraceae, and Thelephoraceae families exhibited north-temperate distribution (15.28%), while Strobilomycetaceae, Entolomataceae, Marasmiaceae, and Ganodermataceae displayed tropical–subtropical distribution (5.56%). Radulomycetaceae is named undetermined distribution, refers to family with no explicit published data about distribution patterns. No macrofungi with endemic distribution were detected in forests of the Ningxia Autonomous Region.
Figure 5.
Proportion of geographical distribution patterns of macrofungal families in the forests of the Ningxia Autonomous Region.
3.5.2. Genera in Funga
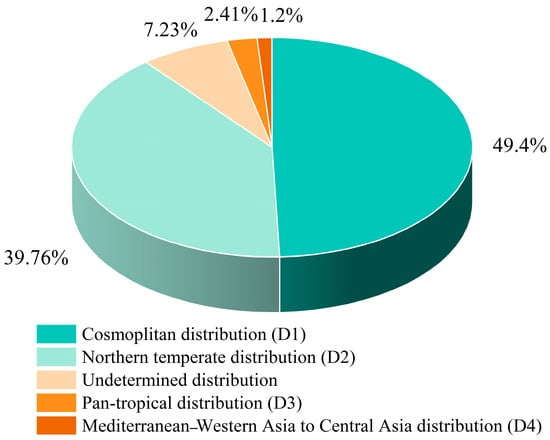
Meanwhile, four geographical distribution patterns were defined for the various genera in this region: cosmopolitan, north-temperate, pan-tropical, and Mediterranean–Western Asian to Central Asian distribution (Figure 6).
Figure 6.
Proportion of geographical distribution patterns of macrofungal genera in the forests of the Ningxia Autonomous Region.
- (1)
- Cosmopolitan (D1)
Cosmopolitan indicates that the genera are distributed across all the world. A total of 78 genera of the Ningxia macrofungi (49.4% of total genera), including Mycena, Lepista, Psathyrella, Agaricus, Russula, Gymnopus, Polyporus, Stropharia, Melanoleuca, Amanita, Clitocybe, Pluteus, Fomitopsis, Lepiota, Daedaleopsis, Oxyporus, Armillaria, Trametes, Calvatia, Clavariadelphus, Cordyceps, Daldinia, Heterobasidion, Lycoperdon, Tremella, Xylaria, Fomitiporia, and Fuscoporia showed cosmopolitan distribution.
- (2)
- North-temperate (D2)
North-temperate indicates that the genera are widely distributed in the northern hemisphere’s temperate regions (Eurasia Continent and North America). Here, 64 genera (39.76% of total genera), including Inocybe, Helvella, Lactarius, Hebeloma, Gomphidius, Cortinarius, Tricholoma, Agrocybe, Clavulina, Ramaria, Suillellus, Hygrophorus, Pseudoclitocybe, Leccinum, Diplomitoporus, Clitopaxillus, Cudonia, Calocybe, Geastrum, Humaria, Anellaria, Limacella, Nigroboletus, Rhizopogon, Xerocomus, Pseudoclitopilus, Exidia, and Phellinus showed north-temperate distribution.
- (3)
- Pan-tropical (D3)
Pan-tropical indicates that the genera are distributed in the tropics of the eastern and western hemispheres, extending to the subtropical to temperate regions but still centered around the tropics. Only Entoloma, Marasmius, Ganoderma, and Xylodon (four genera; 2.41% of total genera) showed pan-tropical distribution in Ningxia Autonomous Region.
- (4)
- Mediterranean–Western Asian to Central Asian (D4)
Mediterranean–Western Asian to Central Asian indicates that the genera are distributed around the Mediterranean region, passing through West Asia–Southwest Asia–Xinjiang–Qinghai Tibet Plateau and the Mongolian Plateau. Among the various macrofungi, only Skeletocutis showed this distribution pattern (1.2% of total genera) in the Ningxia forest.
The final group, named undetermined distribution, refers to genera with no explicit published data about distribution patterns. In the forests of the Ningxia Autonomous Region, Hypholoma, Postia, Spodocybe, Stereopsis, Tephrocybe, Echinoderma, Tomentella, Skvortzovia, Vuilleminia, and Rugosomyces were grouped into this category.
4. Discussion
The current comprehensive study revealed a high macrofungal diversity in the forests of the Ningxia Autonomous Region. We identified 468 species from 157 genera, 72 families, 18 orders, 11 classes, and 2 phyla in the Ningxia forests. We found that the Basidiomycota phylum (437 species) dominated the Ningxia macrofungi, which is consistent with previous reports on the dominant phylum in forests [50].
Many studies on the diversity of macrofungi have been carried out in different regions of China [51,52,53,54,55,56,57]. A total of 345 species were identified in the Taihang Mountains of North China, belonging to 138 genera, 64 families, and 2 phyla [51]. Among them, 11 families, including Cortinariaceae, Russulaceae, Polyporaceae, Inocybaceae, Agaricaceae, and Mycenaceae, were the most species-rich; 16 genera, including Cortinarius, Inocybe, Russula, Hebeloma, Agaricus, and Mycena were the most species-rich. A total of 392 species were identified in the Fuyan Nature Reserve of Guizhou province, belonging to 152 genera, 70 families, and 2 phyla [52]. Among them, 11 families, including Russulaceae, Polyporaceae, Omphalotaceae, and Mycenaceae, were the most species-rich; 18 genera, including Russula, Inocybe, Agaricus, Cortinarius, Lactarius, and Mycena, were the most species-rich. Differences in temperature, humidity, and soil conditions in different regions lead to distinctions in macrofungal species composition. However, the results of present and previous studies show that Russulaceae, Polyporaceae, Mycenaceae, Inocybe, Cortinarius, Mycena, Russula, and Agaricus are consistently dominant groups in the forests of different regions of China.
The most species-rich genus in the Ningxia forests was Inocybe. The Inocybe genus is found to be distributed worldwide and includes diverse species. Additionally, all species of the Inocybe genus are ectomycorrhizal fungi that form ectomycorrhizal relationships with various plants, providing them with stronger environmental adaptability [58]. Generally, in an ecosystem, species of the dominant genera play key functions, such as nutrient circulation and energy flow [59]. Therefore, as the dominant genus, Inocybe probably plays a crucial role in maintaining the ecosystem stability of forests in the Ningxia Autonomous Region.
This study found significant differences in the macrofungal communities among the different forests of Ningxia. Macrofungi are heterotrophic organisms and, therefore, cannot establish self-sustaining communities; they highly depend on their habitat to survive [60]. Previous studies indicated the significant influence of plant composition on the macrofungal diversity of forests [61]. Plant composition is related to litter composition and soil quality, with great impact on the macrofungal diversity of forests [62]. However, more results have shown that ecological factors, such as vegetation, soil, climate, terrain, rainfall, soil moisture, and air temperature, also substantially impact the structure and diversity of macrofungal communities [63,64,65]. In this study, despite divergences in the macrofungal community, the Helan and Liupan Mountains shared the most macrofungal species and had the highest similarity in species, while the Luo and Liupan Mountains shared the least macrofungal species and displayed the lowest similarity in species. The Helan and Luo Mountains have almost the same plant composition but fewer shared macrofungal species. On the other hand, the Helan and Liupan Mountains, with differences in plant composition, exhibited more shared macrofungal species and the highest similarity. These observations confirm the impact of ecological factors on the structure of macrofungal species.
Furthermore, this study defined 206 species of Ningxia macrofungi as edible and/or medicinal, accounting for 44.02% of the macrofungi in the Ningxia forest. Among these, the greatest number of edible species belonged to the Agaricus genus. Additionally, the Agaricus members were identified as saprophytic species with substantial potential to be domesticated. Another 12 edible species were of the Cortinarius genus, which forms ectomycorrhizal relationships with Picea crassifolia. The Cortinarius spp. are famous for their distinct flavor and abundant nutrition [66]. Despite little possibility of being domesticated, the high yield of edible mushrooms of the Cortinarius genus suggests its utilization to improve the incomes of local people. Thus, the present study unveils the considerable potential of the wild edible and medicinal macrofungi of the Ningxia Autonomous Region.
Analyzing the funga of a region helps explore the origin, evolution, and spatiotemporal distribution patterns of fungi [49,67]. A previous study on the funga of the Helan Mountain revealed an obvious north-temperate distribution [68]. The present study found a distinct cosmopolitan distribution (77.78%) for the macrofungi at the family level in the Ningxia forest. In addition, a few macrofungi exhibited north-temperate distribution (15.28%) and tropical–subtropical distribution (5.56%). Meanwhile, the macrofungi at the genus level showed a distinct cosmopolitan distribution (49.4%) and north-temperate distribution (39.76%), with a little pan-tropical (2.41%) and Mediterranean–Western Asian to Central Asian distribution (1.2%). These observations suggest that the macrofungi in the Ningxia forests exhibit distinct cosmopolitan and north-temperate distribution, with a slight transition from pan-tropical to north-temperate. These preliminary data based on regional works provide a solid foundation for detailed research on the funga of the Ningxia forests.
The importance of macrofungal diversity of forests is often undervalued. Forest macrofungi are significant products with immense value for their ecological and economic roles. This study on the diversity of macrofungi provides data for understanding the macrofungal communities of forests [69]. The identification and analysis of the diversity of macrofungi deserve further attention to preserve bioresources and understand the ecological cycle of forests.
Author Contributions
Sampling, X.D., M.L. and X.Y.; Collection, X.D., M.L., Y.D., X.Z. and Y.Y.; Identification, X.D., Y.D. and Y.Y.; Data curation, X.D., M.L. and Y.Y.; Writing original draft, X.D.; Conceptualizing the study, Z.W.; Funding acquisition, X.D., Z.W. and Y.Y.; Visualization, Z.W.; Writing review and editing, Y.Y. All authors have read and agreed to the published version of the manuscript.
Funding
This research was funded by Natural Science Foundation of Ningxia Hui Autonomous Region (2021AAC03202), the Key Research and Development Program Project of Ningxia Hui Autonomous Region (2022BBF03028), National Natural Science Foundation of China (32370013), Major Projects of Science and Technology in Anhui Province (202203a06020009), and Young Elite Scientists Sponsorship Program by CAST (2023QNRC001).
Institutional Review Board Statement
Not applicable.
Data Availability Statement
All collected specimens in this study have been deposited in the herbarium of North Minzu University (NMU), Yinchun, Ningxia.
Acknowledgments
The authors are very grateful to Lihua Sun for offering parts of the macrofungal specimens of Helan Mountain.
Conflicts of Interest
The authors declare no conflicts of interest.
References
- Hawksworth, D.L.; Lucking, R. Fungal diversity revisited: 2.2 to 3.8 million species. Microbiol. Spectr. 2017, 5, 10–1128. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mueller, G.M.; Schmit, J.P.; Leacock, P.R.; Buyck, B.; Cifuentes, J.; Desjardin, D.E.; Halling, R.E.; Hjortstam, K.; Iturriaga, T.; Larsson, K.H. Global diversity and distribution of macrofungi. Biodivers. Conserv. 2019, 16, 37–48. [Google Scholar] [CrossRef] [Scilit]
- Bosso, L.; Lacatena, F.; Varlese, R.; Nocerino, S.; Cristinzio, G.; Russo, D. Plant pathogens but not antagonists change in soil fungal communities across a land abandonment gradient in a Mediterranean landscape. Acta Oecol. 2017, 78, 1–6. [Google Scholar] [CrossRef] [Scilit]
- Yakop, F.; Taha, H.; Shivanand, P. Isolation of fungi from various habitats and their possible bioremediation. Curr. Sci. 2019, 116, 733–740. [Google Scholar] [CrossRef] [Scilit]
- Dai, Y.C.; Yang, Z.L.; Cui, B.K.; Wu, G.; Yuan, H.S.; Zhou, L.W.; He, S.H.; Ge, Z.W.; Wu, F.; Wei, Y.L.; et al. Diversity and systematics of the important macrofungi in Chinese forests. Mycosystema 2021, 40, 770–805. [Google Scholar] [CrossRef]
- Andlar, M.; Rezic, T.; MarCetko, N.; Kracher, D.; Ludwig, R.; Santek, B. Lignocellulose degradation: An overview of fungi and fungal enzymes involved in lignocellulose degradation. Eng. Life Sci. 2018, 18, 768–778. [Google Scholar] [CrossRef] [Scilit]
- Yuan, Y.; Bian, L.S.; Wu, Y.D.; Chen, J.J.; Wu, F.; Liu, H.G.; Zeng, G.Y.; Dai, Y.C. Species diversity of pathogenic wood-rotting fungi (Agaricomycetes, Basidiomycota) in China. Mycology 2023, 14, 204–226. [Google Scholar] [CrossRef] [Scilit]
- Stuart, E.K.; Plett, K.L. Digging deeper: In search of the mechanisms of carbon and nitrogen exchange in ectomycorrhizal symbioses. Front. Plant Sci. 2020, 10, 1658. [Google Scholar] [CrossRef] [Scilit]
- Niego, A.G.T.; Rapior, S.; Thongklang, N.; Raspé, O.; Hyde, K.D.; Mortimer, P. Reviewing the contributions of macrofungi to forest ecosystem processes and services. Fungal Biol. Rev. 2023, 44, 100294. [Google Scholar] [CrossRef] [Scilit]
- Tedersoo, L.; Bahram, M.; Zobel, M. How mycorrhizal associations drive plant population and community biology. Science 2020, 367, eaba1223. [Google Scholar] [CrossRef] [Scilit]
- Liu, Y.; Li, X.; Kou, Y. Ectomycorrhizal fungi: Participation in nutrient turnover and community assembly pattern in forest ecosystems. Forests 2020, 11, 453. [Google Scholar] [CrossRef] [Scilit]
- Adamo, I.; Dashevskaya, S.; Alday, J.G. Fungal perspective of Pine and Oak colonization in Mediterranean degraded ecosystems. Forests 2022, 13, 88. [Google Scholar] [CrossRef] [Scilit]
- Li, H.; Tian, Y.; Menolli, N.; Ye, L.; Karunarathna, S.C.; Perez-Moreno, J.; Rahman, M.M.; Rashid, M.H.; Phengsintham, P.; Rizal, L.; et al. Reviewing the world’s edible mushroom species: A new evidence-based classification system. Compr. Rev. Food Sci. Food Saf. 2021, 20, 1982–2014. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wu, F.; Zhou, L.W.; Yang, Z.L.; Bau, T.; Li, T.H.; Dai, Y.C. Resource diversity of Chinese macrofungi: Edible, medicinal and poisonous species. Fungal Divers. 2019, 98, 1–76. [Google Scholar] [CrossRef] [Scilit]
- Saha, T.K.; Rahman, T.; Moniruzzaman, M.; Min, T.S.; Hossain, Z. Immuno-physiological effects of dietary reishi mushroom powder as a source of beta-glucan on Rohu, Labeo rohita challenged with Aeromonas veronii. Sci. Rep. 2023, 13, 14652. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, Y. The status, opportunities and challenges of edible fungi industry in China: Develop with Chinese characteristic, realize the dream of powerful mushroom industrial country. J. Fungal Res. 2018, 16, 125–131. [Google Scholar] [CrossRef]
- Govigli, V.M.; Gorriz-Mifsud, E.; Varela, E. Zonal travel cost approaches to assess recreational wild mushroom picking value: Trade-offs between online and onsite data collection strategies. For. Policy Econ. 2019, 102, 51–65. [Google Scholar] [CrossRef] [Scilit]
- Schulp, C.J.E.; Thuiller, W.; Verburg, P.H. Wild food in Europe: A synthesis of knowledge and data of terrestrial wild food as an ecosystem service. Ecol. Econ. 2014, 105, 292–305. [Google Scholar] [CrossRef] [Scilit]
- Li, C.; Xu, S. Edible mushroom industry in China: Current state and perspectives. Appl. Microbiol. Biotechnol. 2022, 106, 3949–3955. [Google Scholar] [CrossRef] [Scilit]
- Deng, X.J.; Liu, P.G.; Chen, J.; Liu, J.L.; Amat, R.; Yan, X.F. Distribution of Tuber in Liupan Mountain and its ecological significance. J. Biol. 2023, 40, 45–50. [Google Scholar] [CrossRef]
- Li, X.W.; Li, T.; Zhu, X.T. Atlas of Bryophytes and Macrofungi in Luoshan, Ningxia; Sun Press: Yinchuan, China, 2019; pp. 267–356. [Google Scholar]
- Li, M.Q.; Yan, X.F.; Ren, Y.F.; Zhou, L.B.; Deng, X.J. A study on diversity of macrofungi in Liupanshan National Nature Reserve, Ningxia. Mycosystema 2023, 40, 770–805. [Google Scholar] [CrossRef]
- Song, G.; Song, L.H.; Wang, L.Y. Atlas of Macrofungi in Helan Mountain, Ningxia; Ningxia Children’s Publishing House: Yinchuang, China, 2011; pp. 20–233. [Google Scholar]
- Li, Y. Study on Picea crassifolia Dynamics and Regeneration in the Eastern Slope of Helan Mountain. Master’s Thesis, Northwest A&F University, Xian, China, 2013; pp. 1–96. [Google Scholar]
- Cao, B.; Wang, Z.P. Comprehensive Scientific Investigation of Luoshan National Nature Reserve in Ningxia; Sun Press: Yinchuan, China, 2019; pp. 3–12. [Google Scholar]
- Cheng, J.M. Comprehensive Scientific Investigation of Liupanshan National Nature Reserve, Ningxia; Science Press: Beijing, China, 2013; pp. 3–15. [Google Scholar]
- Reschke, K.; Morozova, O.V.; Dima, B.; Cooper, J.A.; Corriol, G.; Biketova, A.Y.; Piepenbring, M.; Noordeloos, M.E. Phylogeny, taxonomy, and character evolution in Entoloma subgenus nolanea. Persoonia 2022, 49, 136–170. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Romano, N.; Lignola, G.P.; Brigante, M.; Bosso, L.; Chirico, G.B. Residual life and degradation assessment of wood elements used in soil bioengineering structures for slope protection. Ecol. Eng. 2016, 90, 498–509. [Google Scholar] [CrossRef] [Scilit]
- Alsohaili, S.A.; Bani-Hasan, B.M. Morphological and molecular identification of fungi isolated from different environmental sources in the Northern Eastern desert of Jordan. Jordan J. Biol. Sci. 2018, 11, 329–337. [Google Scholar]
- Li, Y.; Li, T.H.; Yang, Z.L.; Bau, T.; Dai, Y.C. Atlas of Chinese Macrofungal Resources; Zhongyuan Farmers Press: Zhengzhou, China, 2015; pp. 25–1300. [Google Scholar]
- Feng, B.; Yang, Z.L. Studies on diversity of higher fungi in Yunnan, southwestern China: A review. Plant Divers. 2018, 40, 31–37. [Google Scholar] [CrossRef] [Scilit]
- Cui, B.K.; Li, H.J.; Ji, X.; Zhou, J.L.; Song, J.; Si, J.; Yang, Z.L.; Dai, Y.C. Species diversity, taxonomy and phylogeny of Polyporaceae (Basidiomycota) in China. Fungal Divers. 2019, 97, 137–392. [Google Scholar] [CrossRef] [Scilit]
- Wu, F.; Yuan, H.S.; Zhou, L.W.; Yuan, Y.; Cui, B.K.; Dai, Y.C. Polypore diversity in south China. Mycosystema 2020, 39, 653–682. [Google Scholar] [CrossRef]
- Bau, T.; Na, Q.; Liu, L.Y. A Monogrph of Mycenaceae (Agaricales) in China; Science Press: Beijing, China, 2021; pp. 20–163. [Google Scholar]
- Cui, Y.Y.; Ding, X.X.; Kost, G.; Yang, Z.L. Tricholoma sect. Tricholoma (Tricholomataceae) from China: Molecular phylogeny and taxonomy. Mycol. Prog. 2022, 21, 35. [Google Scholar] [CrossRef] [Scilit]
- Liimatainen, K.; Kim, J.T.; Pokorny, L.; Kirk, P.M.; Dentinger, B.; Niskanen, T. Taming the beast: A revised classification of Cortinariaceae based on genomic data. Fungal Divers. 2022, 112, 89–170. [Google Scholar] [CrossRef] [Scilit]
- Qi, Y.; Xu, A.; Zhou, Y.; Qin, W.Q.; Guo, H.B.; Yu, X.D. Morphological and Phylogenetic Studies of Three New Species of Calocybe (Agaricales, Basidiomycota) from China. Diversity 2022, 14, 643. [Google Scholar] [CrossRef] [Scilit]
- Xie, M.L.; Phukhamsakda, C.; Wei, T.Z.; Li, J.P.; Wang, K.; Wang, Y.; Ji, R.Q.; Li, Y. Morphological and phylogenetic evidence reveal five new telamonioid species of Cortinarius (Agaricales) from East Asia. J. Fungi 2022, 8, 257. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tie, L.; Lang, Z.; Deng, L.; Zhao, J.Q. Studies on macrofungi diversity and discovery of new species of Abortiporus from Baotianman World Biosphere Reserve. Open Life Sci. 2023, 18, 20220614. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gardes, M.; Bruns, T.D. ITS primers with enhanced specificity for basidiomycetes-application to the identification of mycorrhizae and rusts. Mol. Ecol. 1993, 2, 113–118. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- White, T.J.; Bruns, T.; Lee, S.; Taylor, J. Amplification and direct sequencing of fungal ribosomal RNA genes for phylogenetics. In PCR Protocols: A Guide to Methods and Applications; Innis, M.A., Gelfand, D.H., Sninsky, J.J., White, T.J., Eds.; Academic: New York, NY, USA, 1990; pp. 315–322. [Google Scholar] [CrossRef] [Scilit]
- Liu, S.; Chen, Y.Y.; Sun, Y.F.; He, X.L.; Song, C.G.; Si, J.; Liu, D.M.; Gates, G.; Cui, B.K. Systematic classification and phylogenetic relationships of the brown-rot fungi within the Polyporales. Fungal Divers. 2023, 118, 1–94. [Google Scholar] [CrossRef] [Scilit]
- Vidal, J.M.; Cseh, P.; Merényi, Z.; Bóna, L.; Rudnóy, S.; Bratek, Z.; Paz, A.; Mleczko, P.; Kozak, M.; Chachula, P.; et al. The genus Gautieria (Gomphales) in Europe and the Mediterranean Basin: A morphological and phylogenetic taxonomic revision. Persoonia 2023, 50, 48–122. [Google Scholar] [CrossRef] [Scilit]
- Bau, T.; Li, Y. Study on fungal flora diversity in Daqinggou Nature Reserve. Chin. Biodivers. 2000, 8, 73–80. [Google Scholar] [CrossRef]
- Gryta, A.; Frąc, M. Methodological aspects of multiplex terminal restriction fragment length polymorphism-technique to describe the genetic diversity of soil bacteria, archaea and fungi. Sensors 2020, 20, 3292. [Google Scholar] [CrossRef] [Scilit]
- Kuhar, F.; Furci, G.; Drechsler-Santos, E.R. Delimitation of Funga as a valid term for the diversity of fungal communities: The Fauna, Flora & Funga proposal (FF&F). IMA Fungus 2018, 9, 71–74. [Google Scholar] [CrossRef] [Scilit]
- Sun, B.Y.; Wu, Y.D.; Yuan, Y. Species diversity and floral characteristics of wood-inhabiting macrofungi growing on Quercus mongolica in Northeast China. Mycosystema 2022, 42, 278–289. [Google Scholar] [CrossRef]
- Yang, Y.; Zhao, L.; Chen, Y.L.; Lin, Y.L.; Zhang, L.P.; Luan, F.G.; Wu, P.; Huo, G.H.; Yan, J.Q. Diversity and flora of macrofungi in the Fuheyuan Nature Reserve in Jiangxi Province. J. Northwest For. Univ. 2022, 37, 164–169. [Google Scholar] [CrossRef]
- Zhao, H.; Wu, Y.D.; Yang, Z.R.; Liu, H.G.; Wu, F.; Dai, Y.C.; Yuan, Y. Polypore funga and species diversity in tropical forest ecosystems of Africa, America and Asia, and a comparison with temperate and boreal regions of the Northern Hemisphere. For. Ecosyst. 2024, 11, 100200. [Google Scholar] [CrossRef] [Scilit]
- Izati, N.; Sugiyarto; Purwoko, T. Diversity and distribution of macrofungi in pine forest and mixed forest in Mount Merbabu National Park. In Proceedings of the International Conference on Forest Products (ICFP) 2020: 12th International Symposium of IWORS, Bogor, Indonesia, 1 September 2020; IOP Publishing Ltd.: Bristol, UK, 2020; Volume 935, p. 012030. [Google Scholar] [CrossRef] [Scilit]
- Wang, K.; Du, Z.; Guo, Y.B.; Liu, T.Z.; Xie, M.L.; Zhao, M.J.; Liu, D.M.; Li, G.J.; Wei, T.Z. Diversity of macrofungi in Taihang Mountains of Beijing and Hebei, North China. Mycosystema 2024, 43, 230311. [Google Scholar] [CrossRef]
- Yang, Y.S.; Wang, W.K.; Deng, C.Y.; Han, Y.F. Diversity of Macrofungi in Guizhou Fuyan Nature Reserve. Mycosystema 2024. [Google Scholar] [CrossRef]
- Zheng, H.F.; Shao, Y.Y.; Huang, H.S.; Wei, Q.L.; Huang, F.C.; Liu, B. Macrofungal diversity of White-headed Langurs Nature Reserve in Chongzuo, Guangxi, South China. Mycosystema 2024, 43, 240043. [Google Scholar] [CrossRef]
- Zhang, M.X.; Wang, Z.B.; Zhang, X.; Xi, Y.Q. Macrofungi resources and ecological distribution in Baishuijiang National Nature Reserve in Gansu province. J. Arid Land Res. Environ. 2019, 33, 152–156. [Google Scholar] [CrossRef]
- Hu, Y.Q.; Li, L.Y.; Liu, X.Z.; Lang, N.; Qi, L.L.; Li, Y. Diversity of macrofungi in the karst area of Sino-Vietnam border in Guangxi, South China. Mycosystema 2024, 43, 240106. [Google Scholar] [CrossRef]
- Wang, J.; Liu, D.M.; Zhang, J.; Wang, M.; Deng, C.Y.; Wen, T.C. 2024. Macrofungal diversity and its characteristics in the western priority area of Wuling Mountains. Mycosystema 2024, 43, 230262. [Google Scholar] [CrossRef]
- Guo, T.; Yang, R.H.; Tang, M.X.; Hou, D.; Sun, X.L.; Wang, L.; Li, Y.; Bao, D.P.; Zhou, X.W. Species diversity of macrofungi in the Mount Huangshan, East China. Mycosystema 2022, 41, 1398–1415. [Google Scholar] [CrossRef]
- Fan, Y.G. Taxonomy and Molecular Phylogeny of Inocybe; Jilin Agricultural University: Changchun, China, 2014; pp. 2–3. [Google Scholar]
- Jia, Y.Y.; Qin, W.H.; Zhang, T. Progress on mechanisms underlying arbuscular mycorrhizal fungi maintaining desert ecosystem stability under climate change. Sci. Bull. 2023, 68, 3172–3184. [Google Scholar] [CrossRef] [Scilit]
- Bahram, M.; Põlme, S.; Kõljalg, U.; Zarre, S.; Tedersoo, L. Regional and local patterns of ectomycorrhizal fungal diversity and community structure along an altitudinal gradient in the Hyrcanian forests of northern Iran. New Phytol. 2012, 193, 465–473. [Google Scholar] [CrossRef] [Scilit]
- Copot, O.; Tănase, C. Substrate properties, forest structure and climate influences wood-inhabiting fungal diversity in broadleaved and mixed forests from Northeastern Romania. For. Syst. 2020, 29, 3. [Google Scholar] [CrossRef] [Scilit]
- Kooch, Y.; Sanji, R.; Tabari, M. The effect of vegetation change in C and N contents in litter and soil organic fractions of a northern Iran temperate forest. Catena 2019, 178, 32–39. [Google Scholar] [CrossRef] [Scilit]
- Tuo, Y.L.; Rong, N.; Hu, J.J.; Zhao, G.P.; Wang, Y.; Zhang, Z.H.; Qi, Z.X.; Li, Y.; Zhang, B. Exploring the relationships between macrofungi diversity and major environmental factors in Wunvfeng National Forest Park in northeast China. J. Fungi 2022, 8, 98. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hu, J.J.; Zhao, G.P.; Tuo, Y.L.; Qi, Z.X.; Yue, L.; Zhang, B.; Li, Y. Ecological factors influencing the occurrence of macrofungi from eastern mountainous areas to the central plains of Jilin province, China. J. Fungi 2022, 8, 871. [Google Scholar] [CrossRef] [Scilit]
- Rakić, M.; Marković, M.; Galić, Z.; Galovic, V.; Karaman, M. Diversity and distribution of macrofungi in protected mountain forest habitats in Serbia and its relation to abiotic factors. J. Fungi 2022, 8, 1074. [Google Scholar] [CrossRef] [Scilit]
- Liu, Z.J.; Ma, Q. Effect of Cortinarius rufoolivaceus polysaccharide combined with 5-fu on antioxidase system in H22 tumor bearing mouse. Ningxia Med. J. 2015, 37, 193–196. [Google Scholar] [CrossRef] [Scilit]
- Kujawska, M.B.; Rudawska, M.; Wilgan, R.; Leski, T. Similarities and differences among soil fungal assemblages in managed forests and formerly managed forest reserves. Forests 2021, 12, 353. [Google Scholar] [CrossRef] [Scilit]
- Sun, L.H.; Song, G.; Wang, L.Y.; Yun, X.F. Geographical components of macrofungal flora in Helan Mountain, Ningxia. J. Arid Land Resour. Environ. 2013, 27, 186–190. [Google Scholar] [CrossRef]
- Bazzicalupo, A.; Goncalves, S.C.; Hebert, R.; Jakob, S.; Justo, A.; Kernaghan, G.; Lebeuf, R.; Malloch, B.; Thorn, R.G.; Walker, A.K. Macrofungal conservation in Canada and target species for assessment: A starting point. Facets 2022, 7, 448–463. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2024 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).