


Abstract
The bulk of the chinstrap penguin (Pygoscelis antarcticus) global population inhabits the Antarctic Peninsula and Scotia Sea, which is a region undergoing rapid environmental changes. Consequently, regional level decreases for this species are widespread. This study aimed to evaluate the level of breeding colony changes in the Antarctic Peninsula and South Orkney Islands, which, roughly, hold 60% of the global chinstrap penguin population. The results indicated that within a period of 40 to 50 years, 62% of colonies underwent decreases, and the majority of colonies experienced decreases over 50%, which is represented by numbers in the range of 2000 to 40,000 pairs. Within three generations’ time, the whole population for the area had experienced decreases of around 30%. These levels of decrease add to the fact that the suspected causes are not likely reversible in the short- to mid-term, calling for increased concern about the conservation of this species.
1. Introduction
The chinstrap penguin (Pygoscelis antarcticus) inhabits the cold waters of the Southern Oceans, with most of its populations being found in the Antarctic Peninsula and Scotia Arc [1]. Populations in the Antarctic Peninsula and South Orkney Islands (FAO areas 48.1 and 48.2, respectively) comprise around 60% of the global populations (Table 1) and have undergone a dramatic decrease [1,2].
Table 1.
Percentage of global chinstrap penguin populations breeding in the Antarctic Peninsula (area 48.1) and South Orkneys (area 48.2). Calculated using data from [1].
Chinstrap penguins have specialized in feeding on Krill, at least during the breeding season [3]; as a consequence, the distribution center of the chinstrap penguin is the area where the Antarctic krill (Euphausia superba) is the most abundant swarming organism [4,5]. Chinstrap penguins’ diet in spring and summer comprises between 95% to 99% of Antarctic krill [6,7,8], and, similarly to the other species of the genus, the different periods of the breeding cycle are highly synchronized with the changes in the availability of Antarctic krill during the summer [9,10,11].
Evidence that Antarctic krill abundance is decreasing in the Antarctic Peninsula are starting to accumulate in the literature. A reduction in density at the northern sectors of the species’ distribution is evident from net [12,13] and acoustic [14,15] sampling, and even from Antarctic krill fishing parameters [16]. The reduction in krill abundance as a response to climate change is regarded as the main factor behind decreases in Pygoscelis penguin populations in the Antarctic Peninsula [17].
Recent studies have shown that the lower availability of krill during the summer results from warming conditions during winter, which is translated in lower breeding success for a chinstrap penguin colony [18], therefore supporting the mechanism proposed in [17]. Mortality during the non-breeding season is also recognized as an important driver of Pygoscelis penguin populations [19,20]. As a counterpoint, gentoo penguins (P. papua), which are the less Antarctic krill-specialized Pygoscelis species, have experienced population increases and range expansion [21], despite some local decreases [22,23] that might have been induced by Antarctic krill fishing [24,25,26].
The last IUCN criteria evaluation for chinstrap penguins in 2020 pointed out that the species does not approach the thresholds for vulnerable under the range size criterion, population size criterion, nor when considering the population trend within the time of three generations [27]. In the same year, a study [1] indicated that the majority of chinstrap penguin populations (those with historical data available) have decreased more than 60% over ≈40 years, placing the global population as moderately depleted in the Green Status Assessment [27]. Therefore, this study aims to evaluate breeding colony trends of chinstrap penguins in the Antarctic Peninsula and South Orkneys by analyzing available data from the years 1960 and 2020 [28], calculate ranges of decrease, and estimate the level of the population change within three generations. The rapid changes that the Antarctic Peninsula has been experiencing in the last decades, including rapid warming [29,30], sea ice retreat [31,32] and increased krill fishery [16,24,25,33], justify a regional evaluation.
2. Materials and Methods
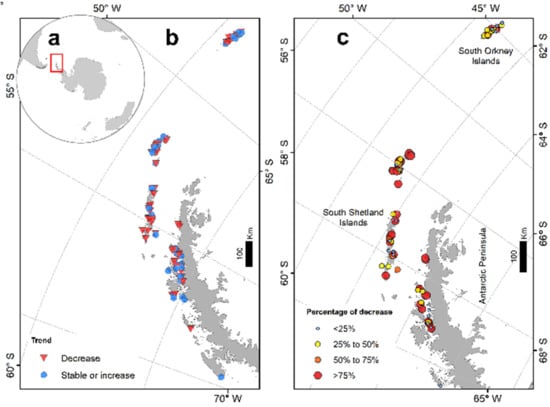
Penguin data were downloaded from the Mapping Application for Penguin Population and Projected Dynamics MAPPPD [28,34]. All data for the areas 48.1 (Antarctic Peninsula) and 48.2 (South Orkney Islands) were downloaded. A total of 133 colonies were used in this study (Figure 1), corresponding to those with a minimum of two counts between 1960 and 2020 (see File S1). Nest counts (breeding pairs) were used as a proxy for colony size and variability.
Figure 1.
Position of the Antarctic Peninsula in the Southern Hemisphere (red square; a) and distribution of the chinstrap penguin (Pygoscelis antarcticus) breeding colonies in the Antarctic Peninsula and South Orkney Islands with a minimum of two counts between 1960 and 2020 (b,c). Trends based on the slope of a site-level generalized linear model with Poisson distribution for counts (b) and percentage of decrease calculated comparing the last with the first available counts (c), only for colonies with slope <0 (decrease on panel ‘b’).
Counts were tested for Poisson distribution using the ‘poisson.mtest’ function in the ‘energy’ R package [35,36], with 199 permutations. Since the data distribution matched a Poisson one (M-CvM = 158.43, p = 0.136), a generalized linear model with Poisson distribution for counts was applied for each colony, in order to identify decreasing (slopes < 0), stable, or increasing (slopes ≥ 0) colonies. Posteriorly, only decreasing colonies were selected to estimate a percent change by comparing the first and last counts. Each colony was classified as being below 25% of decrease, between 25% and 50% of decrease, between 50% and 75% of decrease, and above 75% of decrease.
A generalized linear mixed model using the Markov chain Monte Carlo technique with Poisson distribution was applied using the ‘MCMCglmm’ R package [37,38]. This technique allowed for testing whether a global trend for the temporal variability of the chinstrap colonies throughout the area can be identified by controlling for local differences. The use of a Bayesian approach in a mixed model provides a flexible and robust technique for integrating the random effects of non-Gaussian data [38]. Site ID was entered as a random intercept and the latitude of the breeding colony as a random slope in the model [39]. Additional parameterization can be found in File S1.
The Bayesian GLMM was then used to predict the colony size for all sites between 1960 and 2020. Colonies for all sites were summed for each year to identify the global trend of the population in the area. As the chinstrap penguin generation length is 9.4 years [27], a lagged data frame (27 to 30 year lags, considering ≈3 generations is 28.2 years) was constructed. A percent change was calculated for the lag combinations (0:27 to 0:30).
All analyses were run in R [40]. For detailed methods and codes, please see File S1.
3. Results
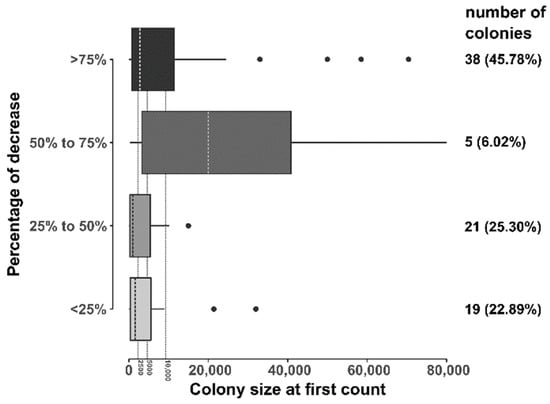
A total of 83 out of 133 colonies (62%) experienced decreases when comparing the first and the last counts (Figure 1a). Colonies that decreased > 75% (Figure 1b) represented the majority (46%), with the colony size predominantly between 2000 and 10,000 nests (Figure 2). Very large colonies (>10,000 nests) predominantly had decreases in the range of 50% to 75% (Figure 2), but these only represented 6% of colonies. Most colonies that presented decreases <50% were those with less than 5000 pairs.
Figure 2.
Percentage of change of the 83 colonies of chinstrap penguins (Pygoscelis antarcticus) breeding populations in the Antarctic Peninsula and South Orkney Islands that had undergone decreases in the period between 1960 and 2020, and the colony size from the first count.
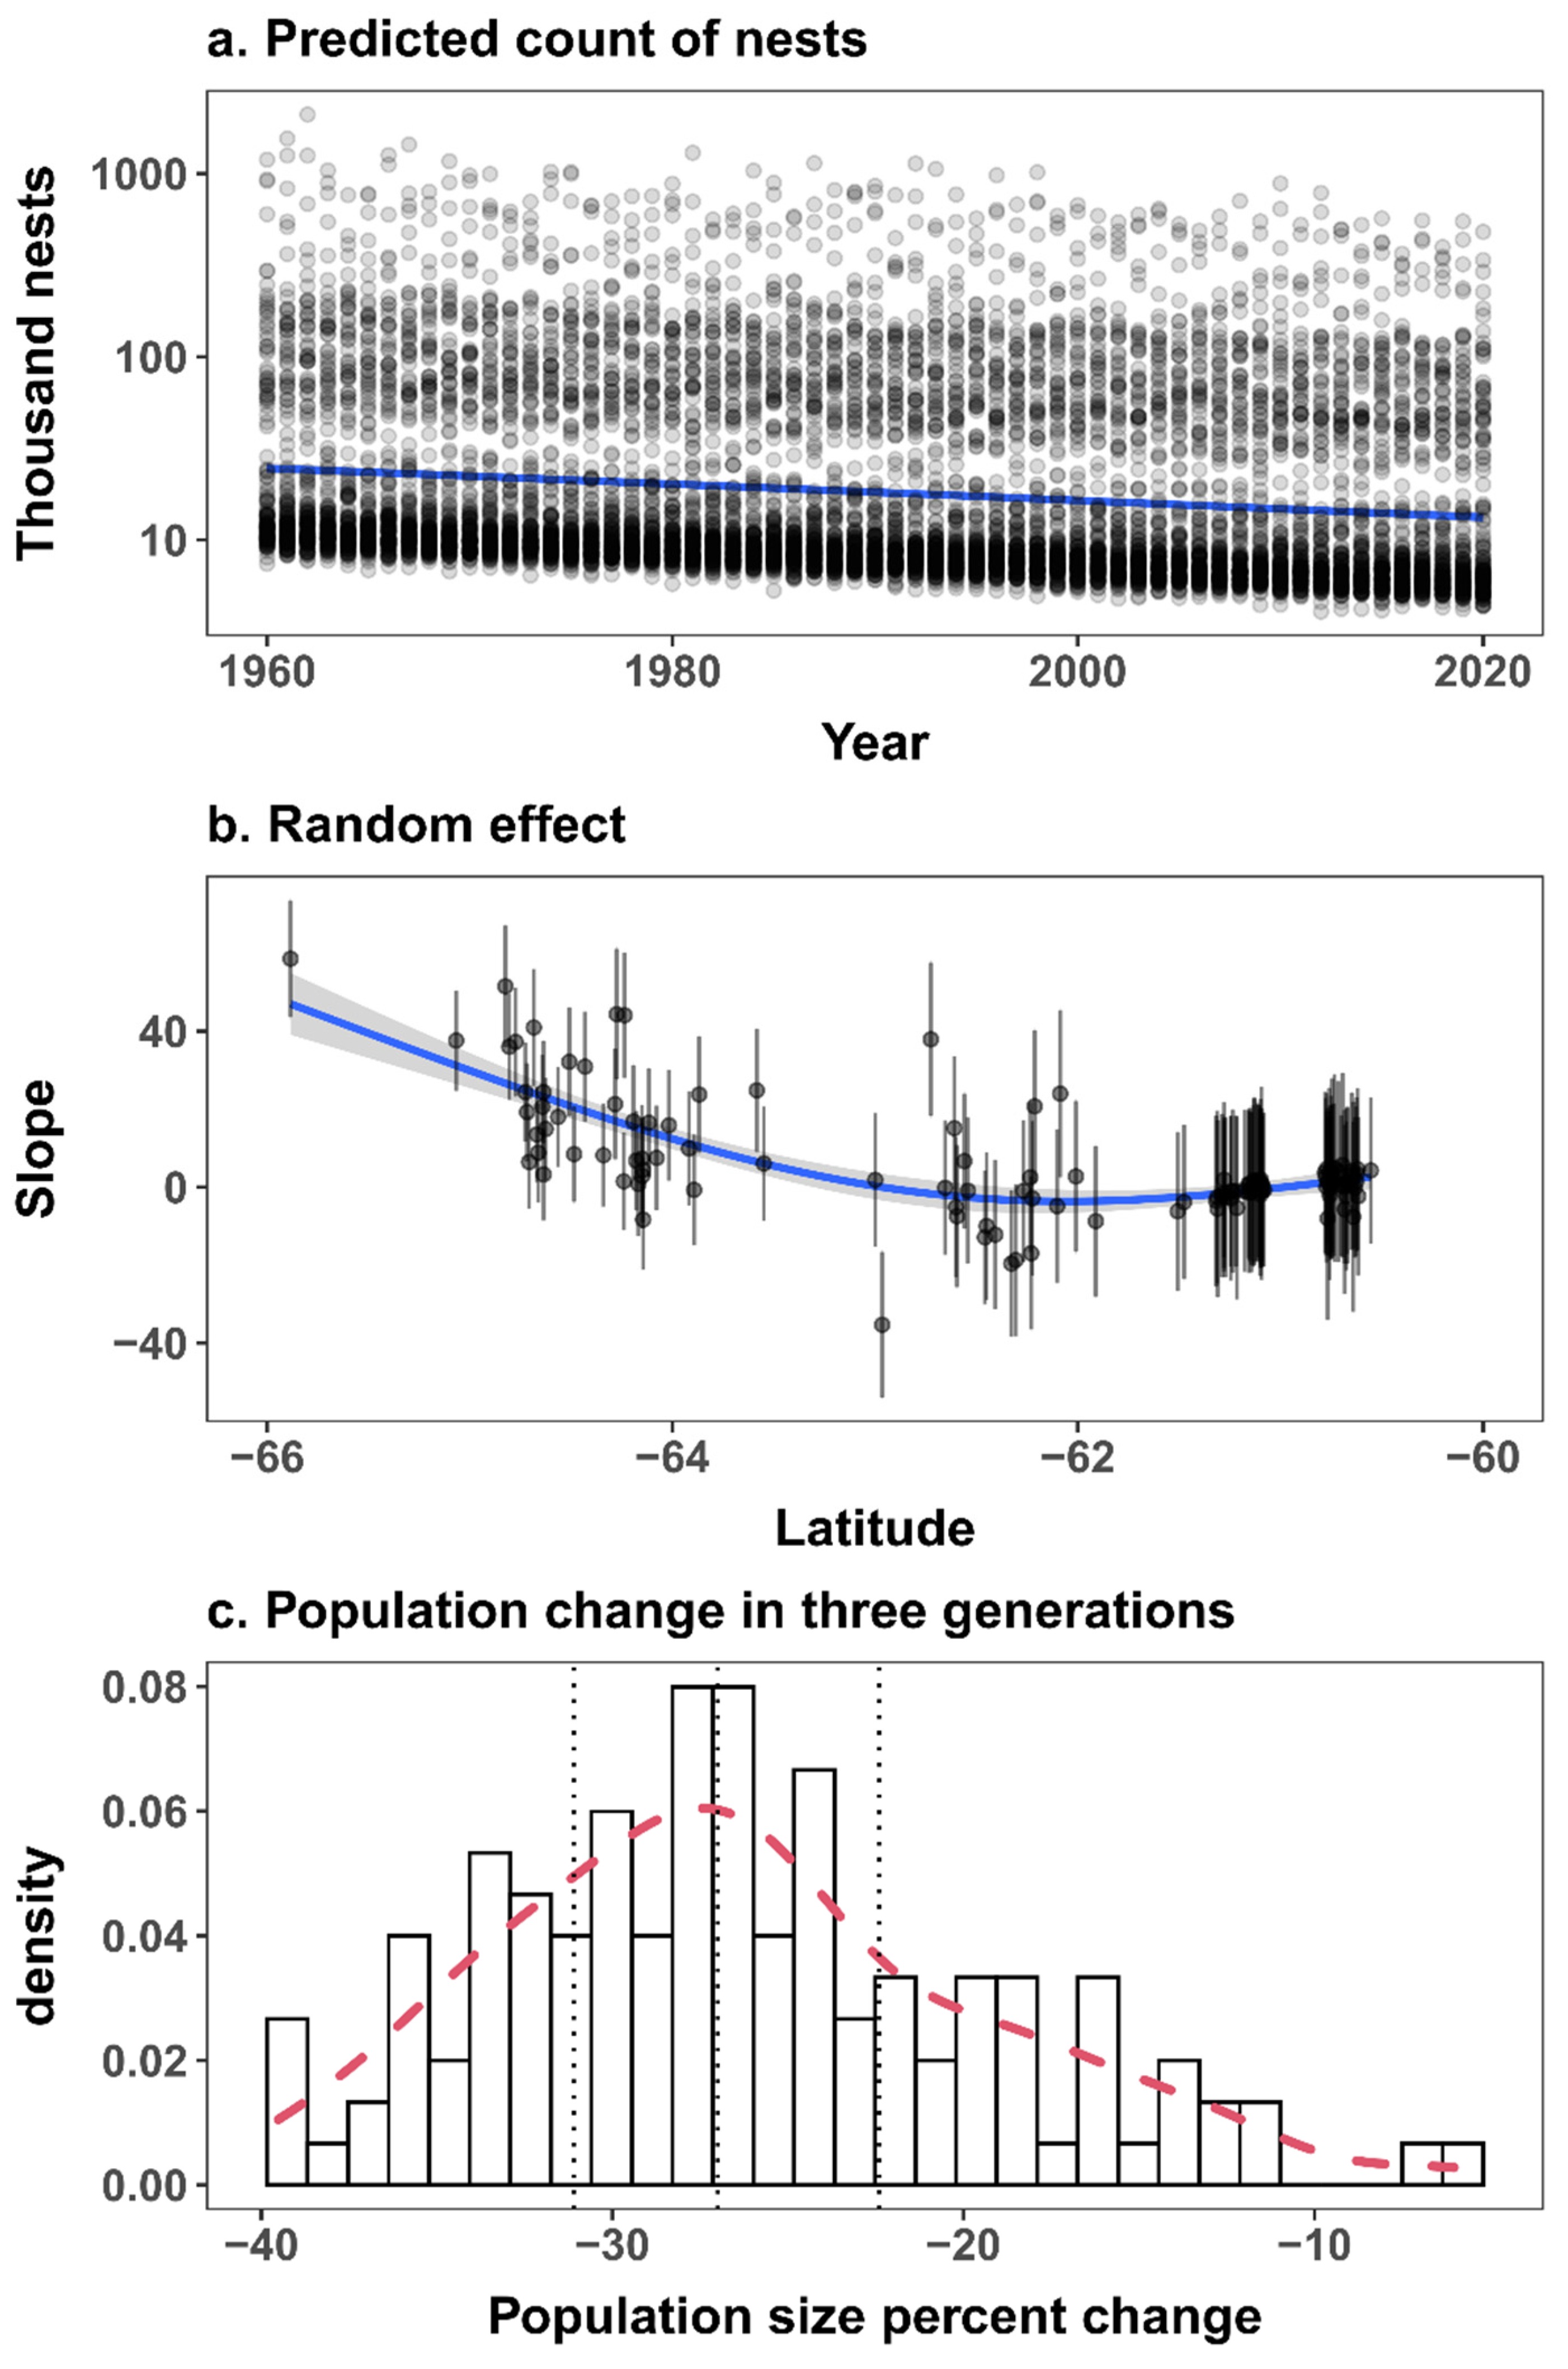
The chinstrap colonies significantly decreased throughout the area (DIC = 4786.3, β = −0.011, eff.samp = 1000, p < 0.001; Figure 3a). Random effects explained 29.15% (24.82% for lower 95% confidence interval, 33.89% for the upper 95% confidence interval), indicating colony-level differences of the temporal trend. A latitudinal gradient on the random effect was clear, as colonies from northerly latitudes (north of 63° S) had a smaller slope compared to those that were more southerly (south of 63° S, Figure 3b). The mean percent change at the population level was −23.08% ± 11.26 (1st qu = −61.62%; 3rd qu = 28.33%) and −27.00 ± 6.99% (−36.32% for lower and −13.78% for the upper 95% confidence intervals) when calculated based on the total GLMM-estimated population size for temporal lags between 27 and 30 years, to represent a three-generation window (Figure 3c).
Figure 3.
Predicted variability of the chinstrap penguin (Pygoscelis antarcticus) breeding colonies in the Antarctic Peninsula and South Orkney Islands estimated using a Bayesian generalized linear mixed model with Poisson distribution. (a) Mean ± standard deviation random slope latitudinal variability (b) and frequency distribution of 3-generation percent change of chinstrap penguin population in the Antarctic Peninsula and South Orkney Islands, as estimated using the Bayesian generalized linear mixed model (c).
4. Discussion
Similarly to results in other studies [1,2,41], this study identified a generalized decrease in chinstrap penguins in the Antarctic Peninsula and a clear latitudinal difference in the level of such a decrease, where southerly colonies were more likely to have stable or increasing trends. Within 40 to 60 years, most colonies have experienced decreases above 50% ([1]; [this study]), and within three generations, decreases predominated near 30% [this study]. Such levels of decrease are consistent with the IUCN criteria A2 for vulnerable species (Table 2). However, some of the larger colonies on the South Sandwich Islands (out of this study analysis) do not have historical data for a proper evaluation of change [1]. However, considering the environmental change factors taking place in the area [29,30,31], such trends are likely to be similar throughout the whole South Atlantic.
Table 2.
Applying the IUCN Red List vulnerable criteria ([42]) for the chinstrap penguin (Pygoscelis antarcticus) breeding populations in the Antarctic Peninsula and South Orkney Islands.
While it was not the aim of this study to evaluate which factors are behind chinstrap penguin trends, other studies have pointed out that changes in marine productivity might be responsible for such geographical differences [2,19]. A proposed mechanism is that lower winter sea ice cover or early sea ice melting would affect krill recruitment by reducing winter habitat for juveniles and/or reducing spring algal bloom [11,18,33]. An asynchrony between the peak of algal bloom and the penguins’ chick rearing as a response to lower winter sea ice and early sea ice melting has been recently shown to be a plausible mechanism to explain the reduction in breeding success of a chinstrap population [18]. Such a mechanism is very likely to be happening at different spatial scales throughout the Antarctic Peninsula, which would explain both the levels of population decreases and the latitudinal differences found here and in other studies. Early [17] and recent [15,24,25] studies advocated that under the decreasing density of krill and the current management strategy, krill fishery could represent a source of interference on penguin populations that might be exacerbated by climate change and the increased consumption of krill by recovering whale populations [15,43,44].
The exact or approximate effect of these factors is not completely understood (Table 2); however, as climate change is expected to continue affecting krill population dynamics [44,45,46], the current trend of chinstrap penguin populations should persist in the short- to mid-term. While it is not clear whether the continuing of krill fishery under current levels might exacerbate the effects of climate change over chinstrap penguins [47], considering recent findings [24,25], reductions in krill catch in certain areas [48] during periods of low krill productivity [33] could enhance the resilience of chinstrap penguin populations to climate change. Suppressing impacts from multiple stressors has been proven to allow species to better respond to climate change [49,50].
5. Conclusions
The region evaluated in this study holds around 60% of chinstrap penguin global populations, which are likely experiencing levels of decrease steep enough to classify the species as vulnerable to extinction. While the complete picture for the global population is still unclear, environmental changes in the areas where most chinstrap penguin breeding populations are placed suggest that similar responses could be expected elsewhere, implying that a higher level of concern and, therefore, protection, should be applied to chinstrap penguins.
Supplementary Materials
The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/d15030327/s1, File S1: R codes for the reproduction of the analysis in the paper.
Funding
This research was funded by Instituto Antártico Chileno Programa AMP (24 03 052) and by ANID—Millennium Science Initiative Program—ICN2021_002.
Institutional Review Board Statement
Not applicable.
Data Availability Statement
Data for this study can be found at the Mapping Application for Penguins Population and Projected Dynamics (https://www.penguinmap.com/).
Acknowledgments
This study was supported by the Marine Protected Areas Program of Instituto Antártico Chileno (AMP 24 03 052), and by ANID—Millennium Science Initiative Program (ICN2021_002), through the Millennium Institute Biodiversity of Antarctic and Subantarctic Ecosystems (BASE).
Conflicts of Interest
The author declares no conflict of interest.
References
- Strycker, N.; Wethington, M.; Borowicz, A.; Forrest, S.; Witharana, C.; Hart, T.; Lynch, H.J. A global population assessment of the Chinstrap penguin (Pygoscelis antarctica). Sci. Rep. 2020, 10, 19474. [Google Scholar] [CrossRef] [Scilit]
- Lynch, H.J.; Naveen, R.; Trathan, P.N.; Fagan, W.F. Spatially integrated assessment reveals widespread changes in penguin populations on the Antarctic Peninsula. Ecology 2012, 93, 1367–1377. [Google Scholar] [CrossRef] [Scilit]
- McMahon, K.W.; Michelson, C.I.; Hart, T.; McCarthy, M.D.; Patterson, W.P.; Polito, M.J. Divergent trophic responses of sympatric penguin species to historic anthropogenic exploitation and recent climate change. Proc. Natl. Acad. Sci. USA 2019, 116, 25721–25727. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nicol, S.; Constable, A.J.; Pauly, T.; Hkh, O. Estimates of circumpolar abundance of antarctic krill based on recent acoustic density measurements. CCAMLR Sci. 2000, 7, 87–99. [Google Scholar]
- Atkinson, A.; Siegel, V.; Pakhomov, E.A.; Rothery, P.; Loeb, V.; Ross, R.M.; Quetin, L.B.; Schmidt, K.; Fretwell, P.; Murphy, E.J.; et al. Oceanic circumpolar habitats of Antarctic krill. Mar. Ecol. Prog. Ser. 2008, 362, 1–23. [Google Scholar] [CrossRef] [Scilit]
- Rombolá, E.F.; Marschoff, E.; Coria, N. Inter-annual variability in Chinstrap penguin diet at South Shetland and South Orkneys Islands. Polar Biol. 2010, 33, 799–806. [Google Scholar] [CrossRef] [Scilit]
- Panasiuk, A.; Wawrzynek-Borejko, J.; Musiał, A.; Korczak-Abshire, M. Pygoscelis penguin diets on King George Island, South Shetland Islands, with a special focus on the krill Euphausia superba. Antarct. Sci. 2020, 32, 21–28. [Google Scholar] [CrossRef] [Scilit]
- Dimitrijević, D.; Paiva, V.H.; Ramos, J.A.; Seco, J.; Ceia, F.R.; Chipev, N.; Valente, T.; Barbosa, A. Isotopic niches of sympatric Gentoo and Chinstrap Penguins: Evidence of competition for Antarctic krill? Polar Biol. 2018, 41, 1655–1669. [Google Scholar] [CrossRef] [Scilit]
- Emmerson, L.; Southwell, C.; Clarke, J.; Tierney, M.; Kerry, K. Adélie penguin response parameters signal reduced prey accessibility: Implications for predator–prey response curves. Mar. Biol. 2015, 162, 1187–1200. [Google Scholar] [CrossRef] [Scilit]
- Youngflesh, C.; Jenouvrier, S.; Li, Y.; Ji, R.; Ainley, D.G.; Ballard, G.; Barbraud, C.; Delord, K.; Dugger, K.M.; Emmerson, L.M.; et al. Circumpolar analysis of the Adélie Penguin reveals the importance of environmental variability in phenological mismatch. Ecology 2017, 98, 940–951. [Google Scholar] [CrossRef] [Scilit]
- Nicol, S.; Worby, A.; Leaper, R. Changes in the Antarctic sea ice ecosystem: Potential effects on krill and baleen whales. Mar. Freshw. Res. 2008, 59, 361. [Google Scholar] [CrossRef] [Scilit]
- Atkinson, A.; Hill, S.L.; Pakhomov, E.A.; Siegel, V.; Reiss, C.S.; Loeb, V.J.; Steinberg, D.K.; Schmidt, K.; Tarling, G.A.; Gerrish, L.; et al. Krill (Euphausia superba) distribution contracts southward during rapid regional warming. Nat. Clim. Change 2019, 9, 142–147. [Google Scholar] [CrossRef] [Scilit]
- Atkinson, A.; Hill, S.L.; Reiss, C.S.; Pakhomov, E.A.; Beaugrand, G.; Tarling, G.A.; Yang, G.; Steinberg, D.K.; Schmidt, K.; Edwards, M.; et al. Stepping stones towards Antarctica: Switch to southern spawning grounds explains an abrupt range shift in krill. Glob. Chang. Biol. 2022, 28, 1359–1375. [Google Scholar] [CrossRef] [Scilit]
- WG-ASAM e-group. Results from the WG-ASAM intersessional e-group on Krill biomass estimates from acoustic surveys. In Proceedings of the Working Group on Ecosystem Monitoring and Management-WG-EMM-2021, Hobart, Australia, 5–9 July 2021. [Google Scholar]
- Trathan, P.N.; Warwick-Evans, V.; Young, E.; Friedlaender, A.; Kim, J.; Kokubun, N. The ecosystem approach to management of the Antarctic krill fishery—The ‘devils are in the detail’ at small spatial and temporal scales. J. Mar. Syst. 2022, 225, 103598. [Google Scholar] [CrossRef] [Scilit]
- Santa Cruz, F.; Krüger, L.; Cárdenas, C.A. Spatial and temporal catch concentrations for Antarctic krill: Implications for fishing performance and precautionary management in the Southern Ocean. Ocean Coast. Manag. 2022, 223, 106146. [Google Scholar] [CrossRef] [Scilit]
- Trivelpiece, W.Z.; Hinke, J.T.; Miller, A.K.; Reiss, C.S.; Trivelpiece, S.G.; Watters, G.M. Variability in krill biomass links harvesting and climate warming to penguin population changes in Antarctica. Proc. Natl. Acad. Sci. USA 2011, 108, 7625–7628. [Google Scholar] [CrossRef] [Scilit]
- Salmerón, N. Warming Precludes Lower Biomass of Antarctic Krill in the South Shetland Islands: Consequences for Foraging and Breeding Success of a Chinstrap Penguin Population. Master’s Thesis, University of Ghant, Ghent, Belgium, 2022. [Google Scholar]
- Hinke, J.T.; Salwicka, K.; Trivelpiece, S.G.; Watters, G.M.; Trivelpiece, W.Z. Divergent responses of Pygoscelis penguins reveal a common environmental driver. Oecologia 2007, 153, 845–855. [Google Scholar] [CrossRef] [Scilit]
- Barbosa, A.; Benzal, J.; De León, A.; Moreno, J. Population decline of chinstrap penguins (Pygoscelis antarctica) on Deception Island, South Shetlands, Antarctica. Polar Biol. 2012, 35, 1453–1457. [Google Scholar] [CrossRef] [Scilit]
- Herman, R.; Borowicz, A.; Lynch, M.; Trathan, P.; Hart, T.; Lynch, H. Update on the global abundance and distribution of breeding Gentoo Penguins (Pygoscelis papua). Polar Biol. 2020, 43, 1947–1956. [Google Scholar] [CrossRef] [Scilit]
- Petry, M.V.; Valls, F.C.L.; Petersen, E.S.; Finger, J.V.G.; Krüger, L. Population trends of seabirds at Stinker Point, Elephant Island, Maritime Antarctica. Antarct. Sci. 2018, 30, 220–226. [Google Scholar] [CrossRef] [Scilit]
- Petry, M.V.; Valls, F.C.L.; Petersen, E.D.S.; Krüger, L.; Piuco, R.D.C.; dos Santos, C.R. Breeding sites and population of seabirds on Admiralty Bay, King George Island, Antarctica. Polar Biol. 2016, 39, 1343–1349. [Google Scholar] [CrossRef] [Scilit]
- Krüger, L.; Huerta, M.F.; Santa Cruz, F.; Cárdenas, C.A. Antarctic krill fishery effects over penguin populations under adverse climate conditions: Implications for the management of fishing practices. Ambio 2021, 50, 560–571. [Google Scholar] [CrossRef] [Scilit]
- Watters, G.M.; Hinke, J.T.; Reiss, C.S. Long-term observations from Antarctica demonstrate that mismatched scales of fisheries management and predator-prey interaction lead to erroneous conclusions about precaution. Sci. Rep. 2020, 10, 2314. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ratcliffe, N.; Deagle, B.; Love, K.; Polanowski, A.; Fielding, S.; Wood, A.G.; Hill, S.; Grant, S.; Belchier, M.; Fleming, A.; et al. Changes in prey fields increase the potential for spatial overlap between gentoo penguins and a krill fishery within a marine protected area. Divers. Distrib. 2021, 27, 552–563. [Google Scholar] [CrossRef] [Scilit]
- BirdLife International. Pygoscelis Antarcticus. The IUCN Red List of Threatened Species; BirdLife International: Cambridge, UK, 2020; p. 8235. [Google Scholar]
- Humphries, G.R.W.; Naveen, R.; Schwaller, M.; Che-Castaldo, C.; McDowall, P.; Schrimpf, M.; Lynch, H. Mapping Application for Penguin Populations and Projected Dynamics (MAPPPD): Data and tools for dynamic management and decision support. Polar Rec. 2017, 53, 160–166. [Google Scholar] [CrossRef] [Scilit]
- Bozkurt, D.; Bromwich, D.H.; Carrasco, J.; Hines, K.M.; Maureira, J.C.; Rondanelli, R. Recent Near-surface Temperature Trends in the Antarctic Peninsula from Observed, Reanalysis and Regional Climate Model Data. Adv. Atmos. Sci. 2020, 37, 477–493. [Google Scholar] [CrossRef] [Scilit]
- Carrasco, J.F.; Bozkurt, D.; Cordero, R.R. A review of the observed air temperature in the Antarctic Peninsula. Did the warming trend come back after the early 21st hiatus? Polar Sci. 2021, 28, 100653. [Google Scholar] [CrossRef] [Scilit]
- Eayrs, C.; Li, X.; Raphael, M.N.; Holland, D.M. Rapid decline in Antarctic sea ice in recent years hints at future change. Nat. Geosci. 2021, 14, 460–464. [Google Scholar] [CrossRef] [Scilit]
- Parkinson, C.L. A 40-y record reveals gradual Antarctic sea ice increases followed by decreases at rates far exceeding the rates seen in the Arctic. Proc. Natl. Acad. Sci. USA 2019, 116, 14414–14423. [Google Scholar] [CrossRef] [Scilit]
- Meyer, B.; Atkinson, A.; Bernard, K.S.; Brierley, A.S.; Driscoll, R.; Hill, S.L.; Marschoff, E.; Maschette, D.; Perry, F.A.; Reiss, C.S.; et al. Successful ecosystem-based management of Antarctic krill should address uncertainties in krill recruitment, behaviour and ecological adaptation. Commun. Earth Environ. 2020, 1, 28. [Google Scholar] [CrossRef] [Scilit]
- Lynch, H.; Che-Castaldo, C.; Humphries, G.; Naveen, R. MAPPPD (Mapping Application for Penguin Populations and Projected Dynamics). 2022. Available online: https://www.penguinmap.com/ (accessed on 23 August 2022).
- Rizzo, M.; Szekely, G. E-Statistics: Multivariate Inference vie the Energy of Data; The Comprehensive R Archive Network: Vienna, Austria, 2022. [Google Scholar]
- Rizzo, M.L.; Székely, G.J. Energy distance. Wiley Interdiscip. Rev. Comput. Stat. 2016, 8, 27–38. [Google Scholar] [CrossRef] [Scilit]
- Hadfield, J. MCMC Generalised Linear Mixed Models; The Comprehensive R Archive Network: Vienna, Austria, 2022. [Google Scholar]
- Hadfield, J.D. MCMC Methods for Multi-Response Generalized Linear Mixed Models: The MCMCglmm R Package. J. Stat. Softw. 2010, 33, 1–21. [Google Scholar] [CrossRef] [Scilit]
- Houslay, T.M.; Wilson, A.J. Avoiding the misuse of BLUP in behavioural ecology. Behav. Ecol. 2017, 28, 948–952. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- R Core Team. R: A Language and Environment for Statistical Computing; R Foundation for Statistical Computing: Vienna, Austria, 2022. [Google Scholar]
- Casanovas, P.; Naveen, R.; Forrest, S.; Poncet, J.; Lynch, H.J. A comprehensive coastal seabird survey maps out the front lines of ecological change on the western Antarctic Peninsula. Polar Biol. 2015, 38, 927–940. [Google Scholar] [CrossRef] [Scilit]
- IUCN. IUCN Red List Categories and Criteria: Version 3.1, 2nd ed.; IUCN International Union for Conservation of Nature: Gland, Switzerland; Cambridge, MA, USA, 2012; ISBN 9782831714356. [Google Scholar]
- Green, D.B.; Bestley, S.; Corney, S.P.; Trebilco, R.; Lehodey, P.; Hindell, M.A. Modelling Antarctic Krill Circumpolar Spawning Habitat Quality to Identify Regions with Potential to Support High Larval Production. Geophys. Res. Lett. 2021, 48, e2020GL091206. [Google Scholar] [CrossRef] [Scilit]
- David, C.L.; Schaafsma, F.L.; van Franeker, J.A.; Pakhomov, E.A.; Hunt, B.P.V.; Lange, B.A.; Castellani, G.; Brandt, A.; Flores, H. Sea-Ice Habitat Minimizes Grazing Impact and Predation Risk for Larval Antarctic Krill. Polar Biol. 2021, 44, 1175–1193. [Google Scholar] [CrossRef] [Scilit]
- Veytia, D.; Corney, S.; Meiners, K.M.; Kawaguchi, S.; Murphy, E.J.; Bestley, S. Circumpolar Projections of Antarctic Krill Growth Potential. Nat. Clim. Change 2020, 10, 568–575. [Google Scholar] [CrossRef] [Scilit]
- Sylvester, Z.T.; Long, M.C.; Brooks, C.M. Detecting Climate Signals in Southern Ocean Krill Growth Habitat. Front. Mar. Sci. 2021, 8, 669508. [Google Scholar] [CrossRef] [Scilit]
- Testa, G.; Neira, S.; Giesecke, R.; Piñones, A. Projecting Environmental and Krill Fishery Impacts on the Antarctic Peninsula Food Web in 2100. Prog. Oceanogr. 2022, 206, 102862. [Google Scholar] [CrossRef] [Scilit]
- Godø, O.R.; Trathan, P. Voluntary Actions by the Antarctic Krill Fishing Industry Help Reduce Potential Negative Impacts on Land-Based Marine Predators during Breeding, Highlighting the Need for CCAMLR Action. ICES J. Mar. Sci. 2022, 79, 1457–1466. [Google Scholar] [CrossRef] [Scilit]
- Roberts, C.M.; O’Leary, B.C.; McCauley, D.J.; Cury, P.M.; Duarte, C.M.; Lubchenco, J.; Pauly, D.; Sáenz-Arroyo, A.; Sumaila, U.R.; Wilson, R.W.; et al. Marine Reserves Can Mitigate and Promote Adaptation to Climate Change. Proc. Natl. Acad. Sci. USA 2017, 114, 6167–6175. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wilson, K.L.; Tittensor, D.P.; Worm, B.; Lotze, H.K. Incorporating Climate Change Adaptation into Marine Protected Area Planning. Glob. Change Biol. 2020, 26, 3251–3267. [Google Scholar] [CrossRef] [Scilit] [PubMed]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2023 by the author. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).