


Abstract
In this paper, we discuss the competition of two species for a single essential growth-limiting nutriment with viral infection that affects only the first species. Although the classical models without viral infection suggest competitive exclusion, this model exhibits the stable coexistence of both species. We reduce the fourth-dimension proposed model to a three-dimension one. Thus, the coexistence of the two competing species is demonstrated using the theory of uniform persistence applied to the three-variable reduced system. We prove that there is no coexistence of both species without the presence of the virus and the satisfaction of some assumptions on the growth rates of species. Finally, we give some numerical simulations to confirm the obtained theoretical findings.
MSC:
92A15; 92A17; 34C15; 34C35
1. Introduction
A chemostat is a particular type of bioreactor that permits the continuous cultivation of micro-organisms in an environment which is under control, that is to say, it makes it possible to grow a population of micro-organisms (unicellular algae, bacteria, yeasts, phytoplankton, zooplankton, molds, etc.) on certain substrates, while preserving the surrounding conditions (temperature, brightness, pH, and aeration). It is used for the production of the cell mass itself, for the extraction and degradation of certain pollutants in a liquid medium, for the production of organic substances resulting from the metabolic activity, or for the study of physiological and metabolic processes of micro-organisms in a specific medium. We can, then, by varying the the limiting substrates in a chemostat, study precisely the influence of each substrate on an organism.
The competition between n species for k resources is a subject that has been studied in theoretical ecology. A classical postulate suggests that if , then at least species cannot coexist. This postulate is known as the competitive exclusion principle. In the case of two competing species for a single resource , the competitive exclusion principle means that, at most, one species of micro-organisms is able to survive long term, while the other species should disappear. This principle has been demonstrated mathematically and validated in several experiments. In 1977, Hsu et al. [1] considered n species competing for a single substrate, and they then showed the validity of the competitive exclusion principle. Butler and Wolkowicz [2] showed that the competitive exclusion principle is still valid for non-monotonic growth rates. Wolkowicz and Lu [3] also verified the principle of competitive exclusion by using Lyapunov functions for general growth rates and for different death rates. Smith and Waltman [4] verified the competitive exclusion principle for the Droop model.
One area being considered is the control of the chemostat using a control variable, for example, the input substrate concentration or the dilution rate D. In this way, one places oneself in the case of systems in competition in a variable environment, wherein one knows that they are able to generate a behavior of coexistence. Hsu [5] considered in 1980 the case of competition in a chemostat forced periodically by the concentration of substrate . In a numerical study showing the possibility of coexistence of the competitors, Smith [6] adopted this model in 1981 and showed that coexistence is possible, in the case of two populations. In 1983, Hale and Somolinos [7] extended Smith’s work in the case of n, which is computed in a periodic chemostat, using the dissipativity of the system. They also showed that, despite the periodic forcing, there are ranges of parameters for which the competitive exclusion takes place. Similar approaches were studied in [8,9,10,11,12,13,14,15] in order to explain the coexistence of competing species, in particular, by using the periodic dilution rate and/or periodic input of the substrate [16,17,18], by introducing inhibition [19], considering the case of the competition between two species indifferently using one of two nutrients [20], or by considering the ratio-dependent growth rate [21,22,23,24,25,26].
In [27], Wolkowicz considered a food web in a continuous reactor, where several competitor populations compete for a single, essential, non-reproducing, growth-limiting substrate, and several predator populations prey on some or all of the competitor populations. In [27], the growth functions are assumed to be either Lotka–Volterra (i.e., linear) or Michaelis–Menten. Under some assumptions, the model predicts the asymptotic survival of each of the different populations. In [28], the authors tested a planktonic system composed of a zooplankton predator and multiple algal prey. Their results highlight the importance of considering transient dynamics when assessing the role of stabilizing factors on the dynamics of food webs.
In this paper, we consider a bioreactor in which two species are competing for a single essential growth-limiting nutriment by including a virus that affects only the first species to the competition. The mathematical model proposed here is a particular case of the model studied by Wolkowicz [27] when considering only two species and one virus, but in our case, we take general monotone functional responses. Our model is also considered in [28] with specific growth functions. We conduct an analytic study of the existence and stability of the steady states for general growth rate functions. Thus, the present paper is organized as the following: in Section 2, we present the mathematical model with two species competing for a single nutriment by adding a virus affecting only the first species to the competition, where we considered general smooth microbial growth functions for both species. We give some preliminary results on the positivity and boundedness of trajectories, and we recall some stability results for the model in the absence of the virus. In Section 3, we study the necessary and sufficient conditions for the existence of steady states, then the local stability of the steady states are studied with respect to some operating parameters. In Section 4, we prove that the model is uniformly persistent, i.e., both populations avoid extinction. In Section 5, we discuss some numerical results confirming the obtained theoretical findings. Finally, in Section 6, we give some concluding remarks.
2. Mathematical Model for the Competition in the Presence of a Virus
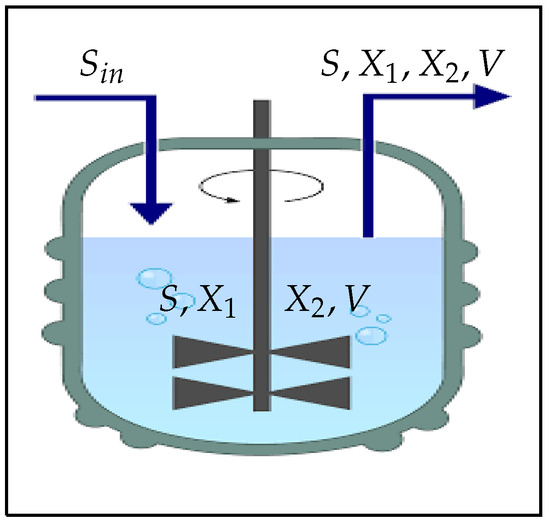
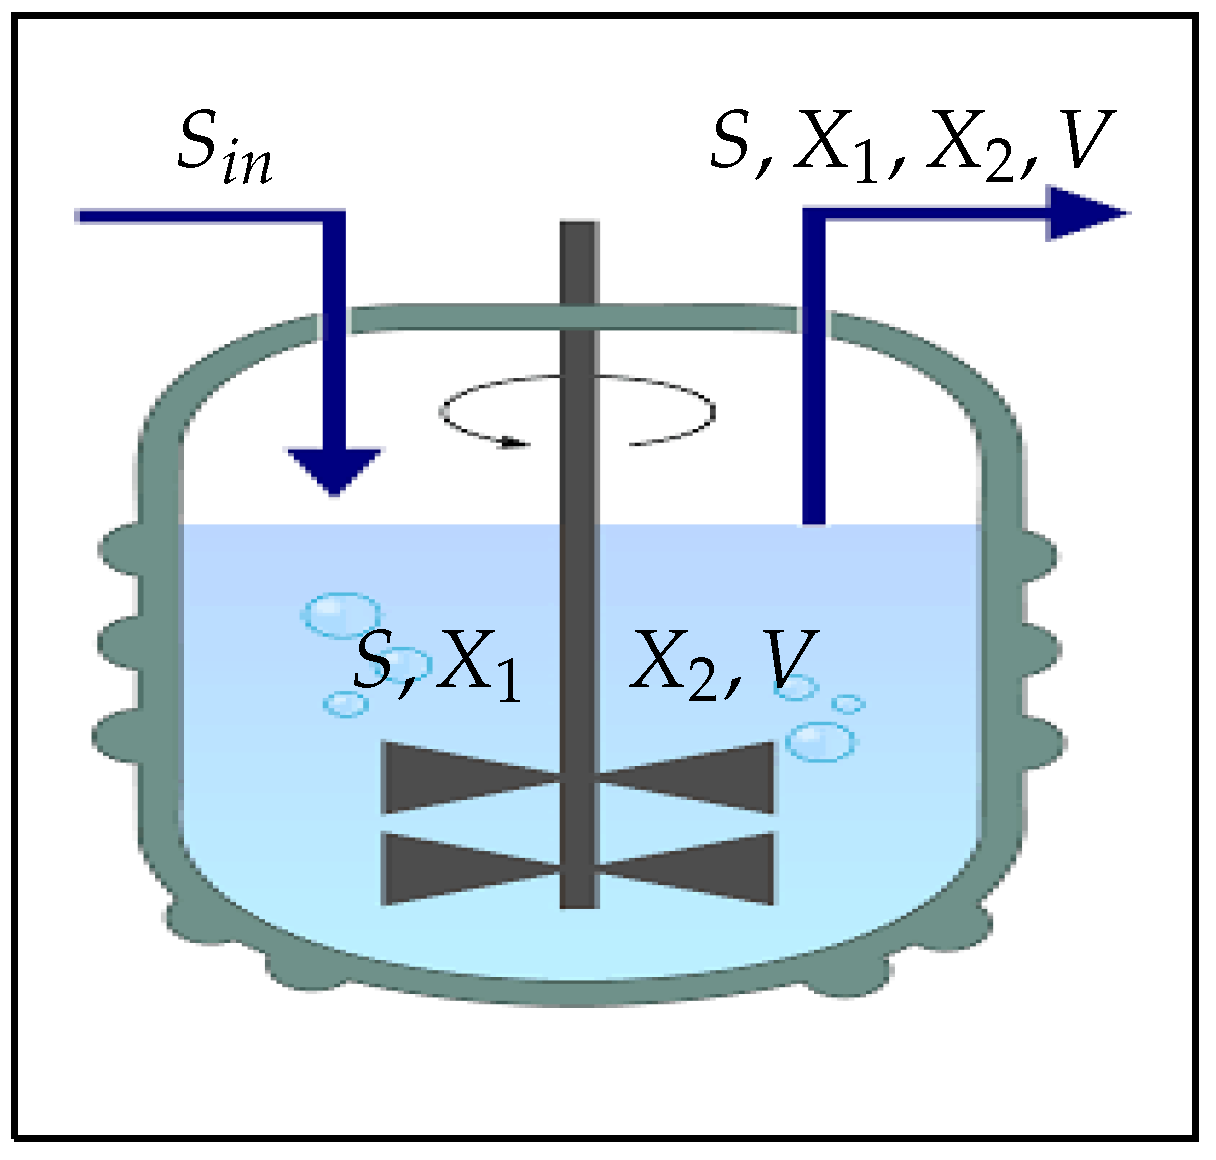
Consider a bioreactor (chemostat), where a limiting nutriment was continuously added at an input concentration (), and the culture liquid () is continuously removed at the same flow rate (D) [22]. The virus, V, was assumed to be associated only with the first species (Figure 1).
Figure 1.
A bioreactor(chemostat) is a continuous stirring mechanism, where a limiting nutriment is continuously added at an input concentration (), and the culture liquid () is continuously removed at the same flow rate (D).
We consider a mathematical model for the chemostat where two bacteria are competing for a unique essential growth-limiting substrate in the presence of a virus associated only with the first species.
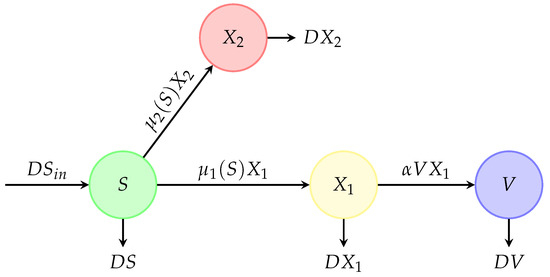
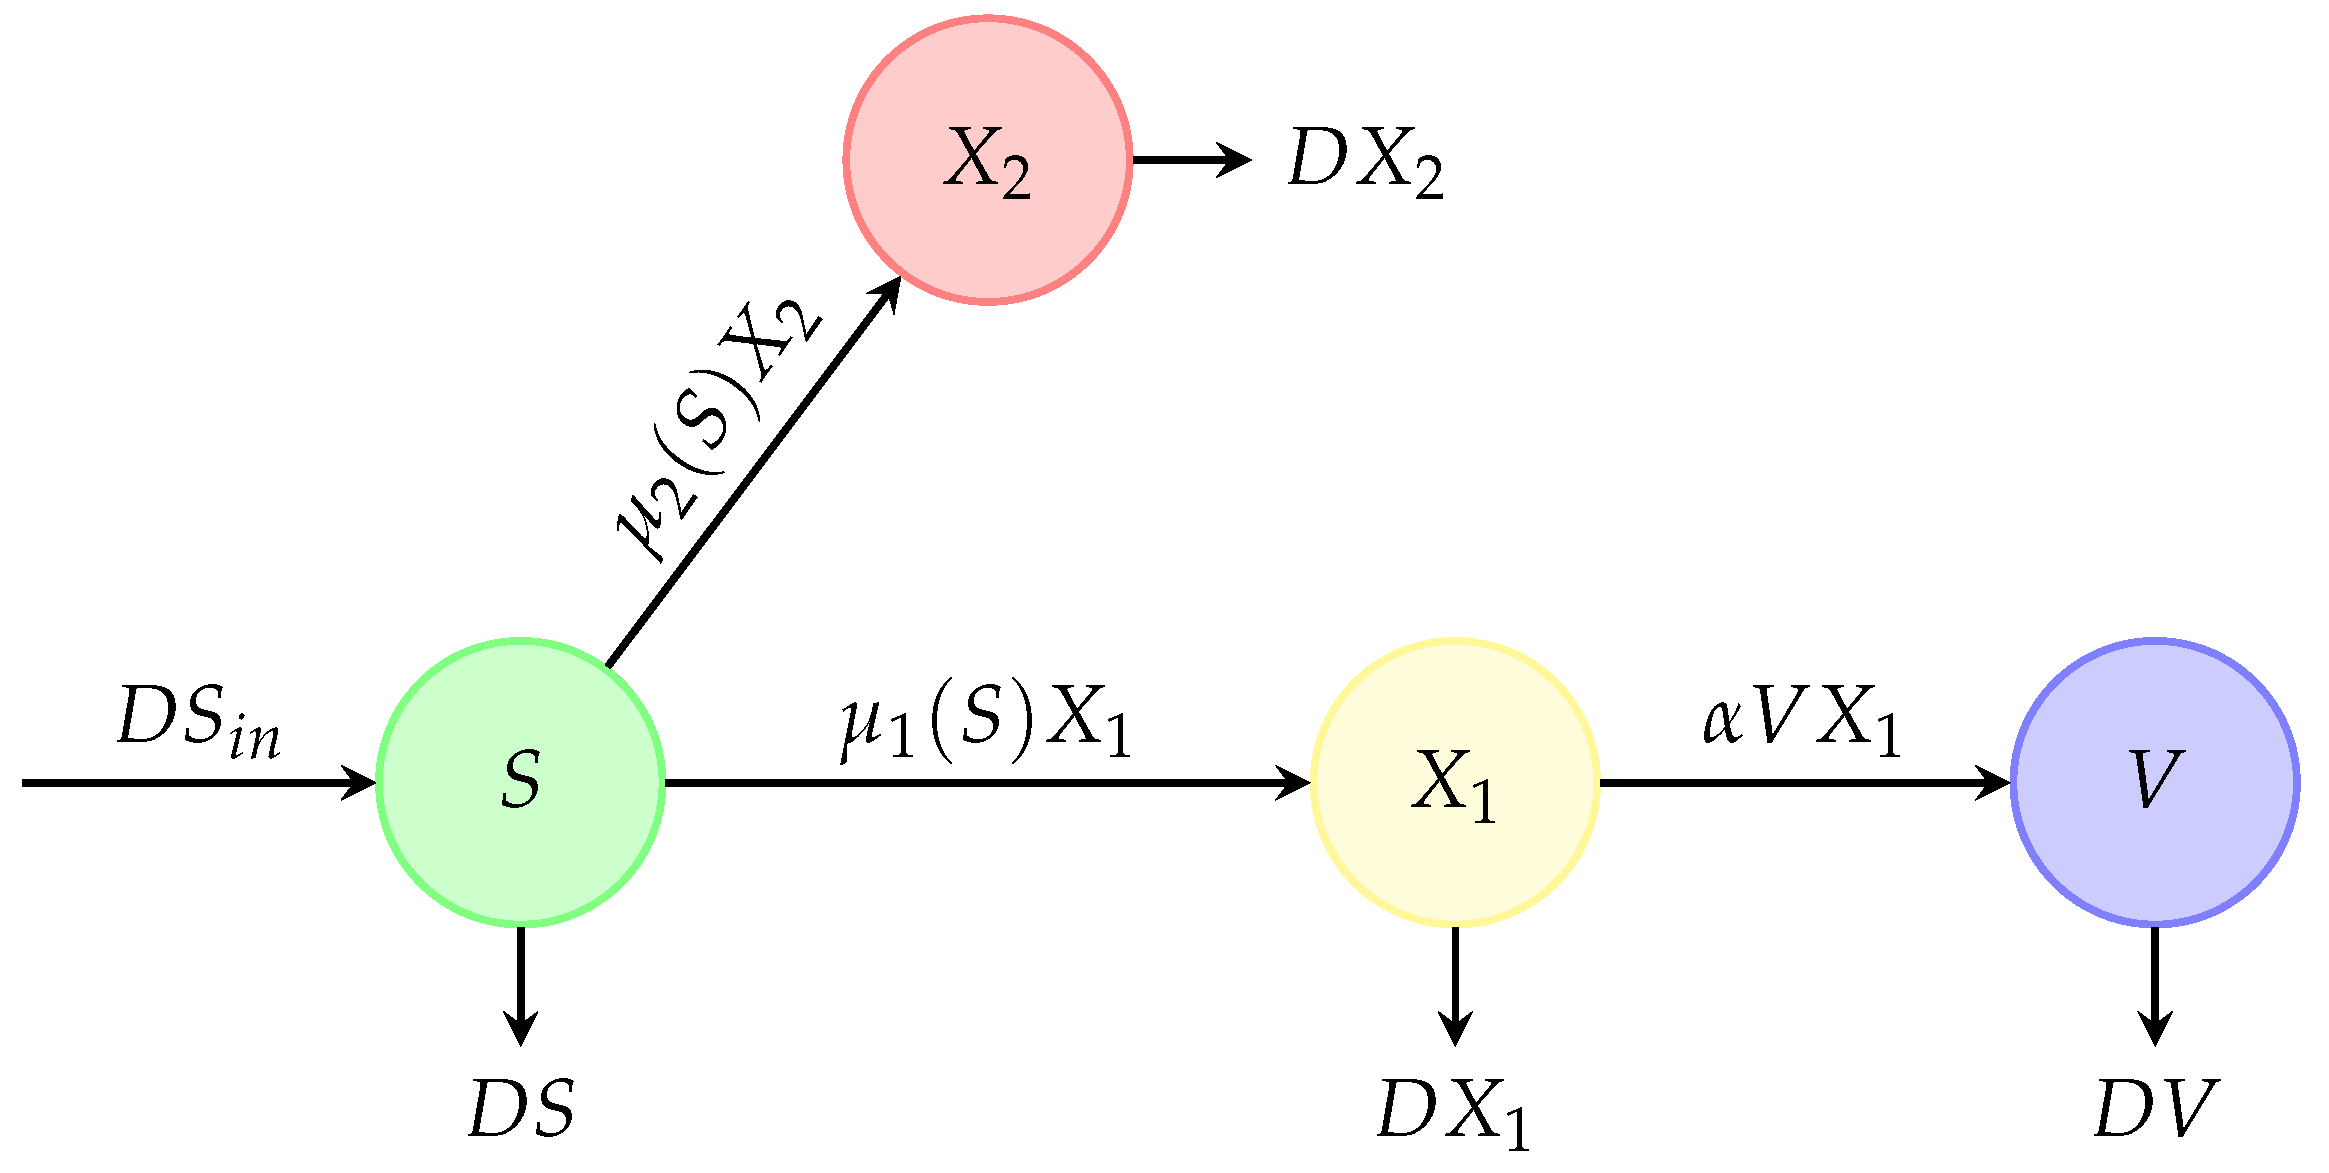
S is the concentration of the nutriment such that , and are the concentrations of each micro-organism, where and . The constant denotes the dilution rate, and the constant denotes the input concentration. and denote the yield coefficients, commonly referred to as the substrate-to-species 1 and substrate-to-species 2 yields, respectively. k denotes the species 1-to-virus yield. and are the specific growth rates of species 1 and species 2, respectively. Each infected species(1) has a fixed number of contacts per unit of time that are sufficient to become infectious (Figure 2).
Figure 2.
Competition of two species in a chemostat in presence of one species virus. Circles describe the compartments and V and the arrows (and labels) correspond to rates of transition between them.
By making the following change of variable, we obtain a more simplified model. Let , and . Then the model takes the form
The growth rates and are non-negative functions such that .
Note that this mathematical model is a particular case of the one studied by Wolkowicz [27] when considering only two species and one virus.
2.1. Fundamental Properties
The chemostat model (2) satisfied some classical properties [29] given here below.
Proposition 1.
Proof.
- is invariant since , for and .Since all compartments of M are non-negative, the trajectory is thus bounded.
□
Corollary 1.
For all , then there exists such that
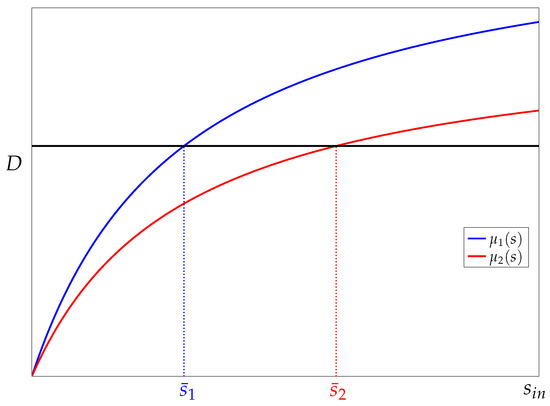
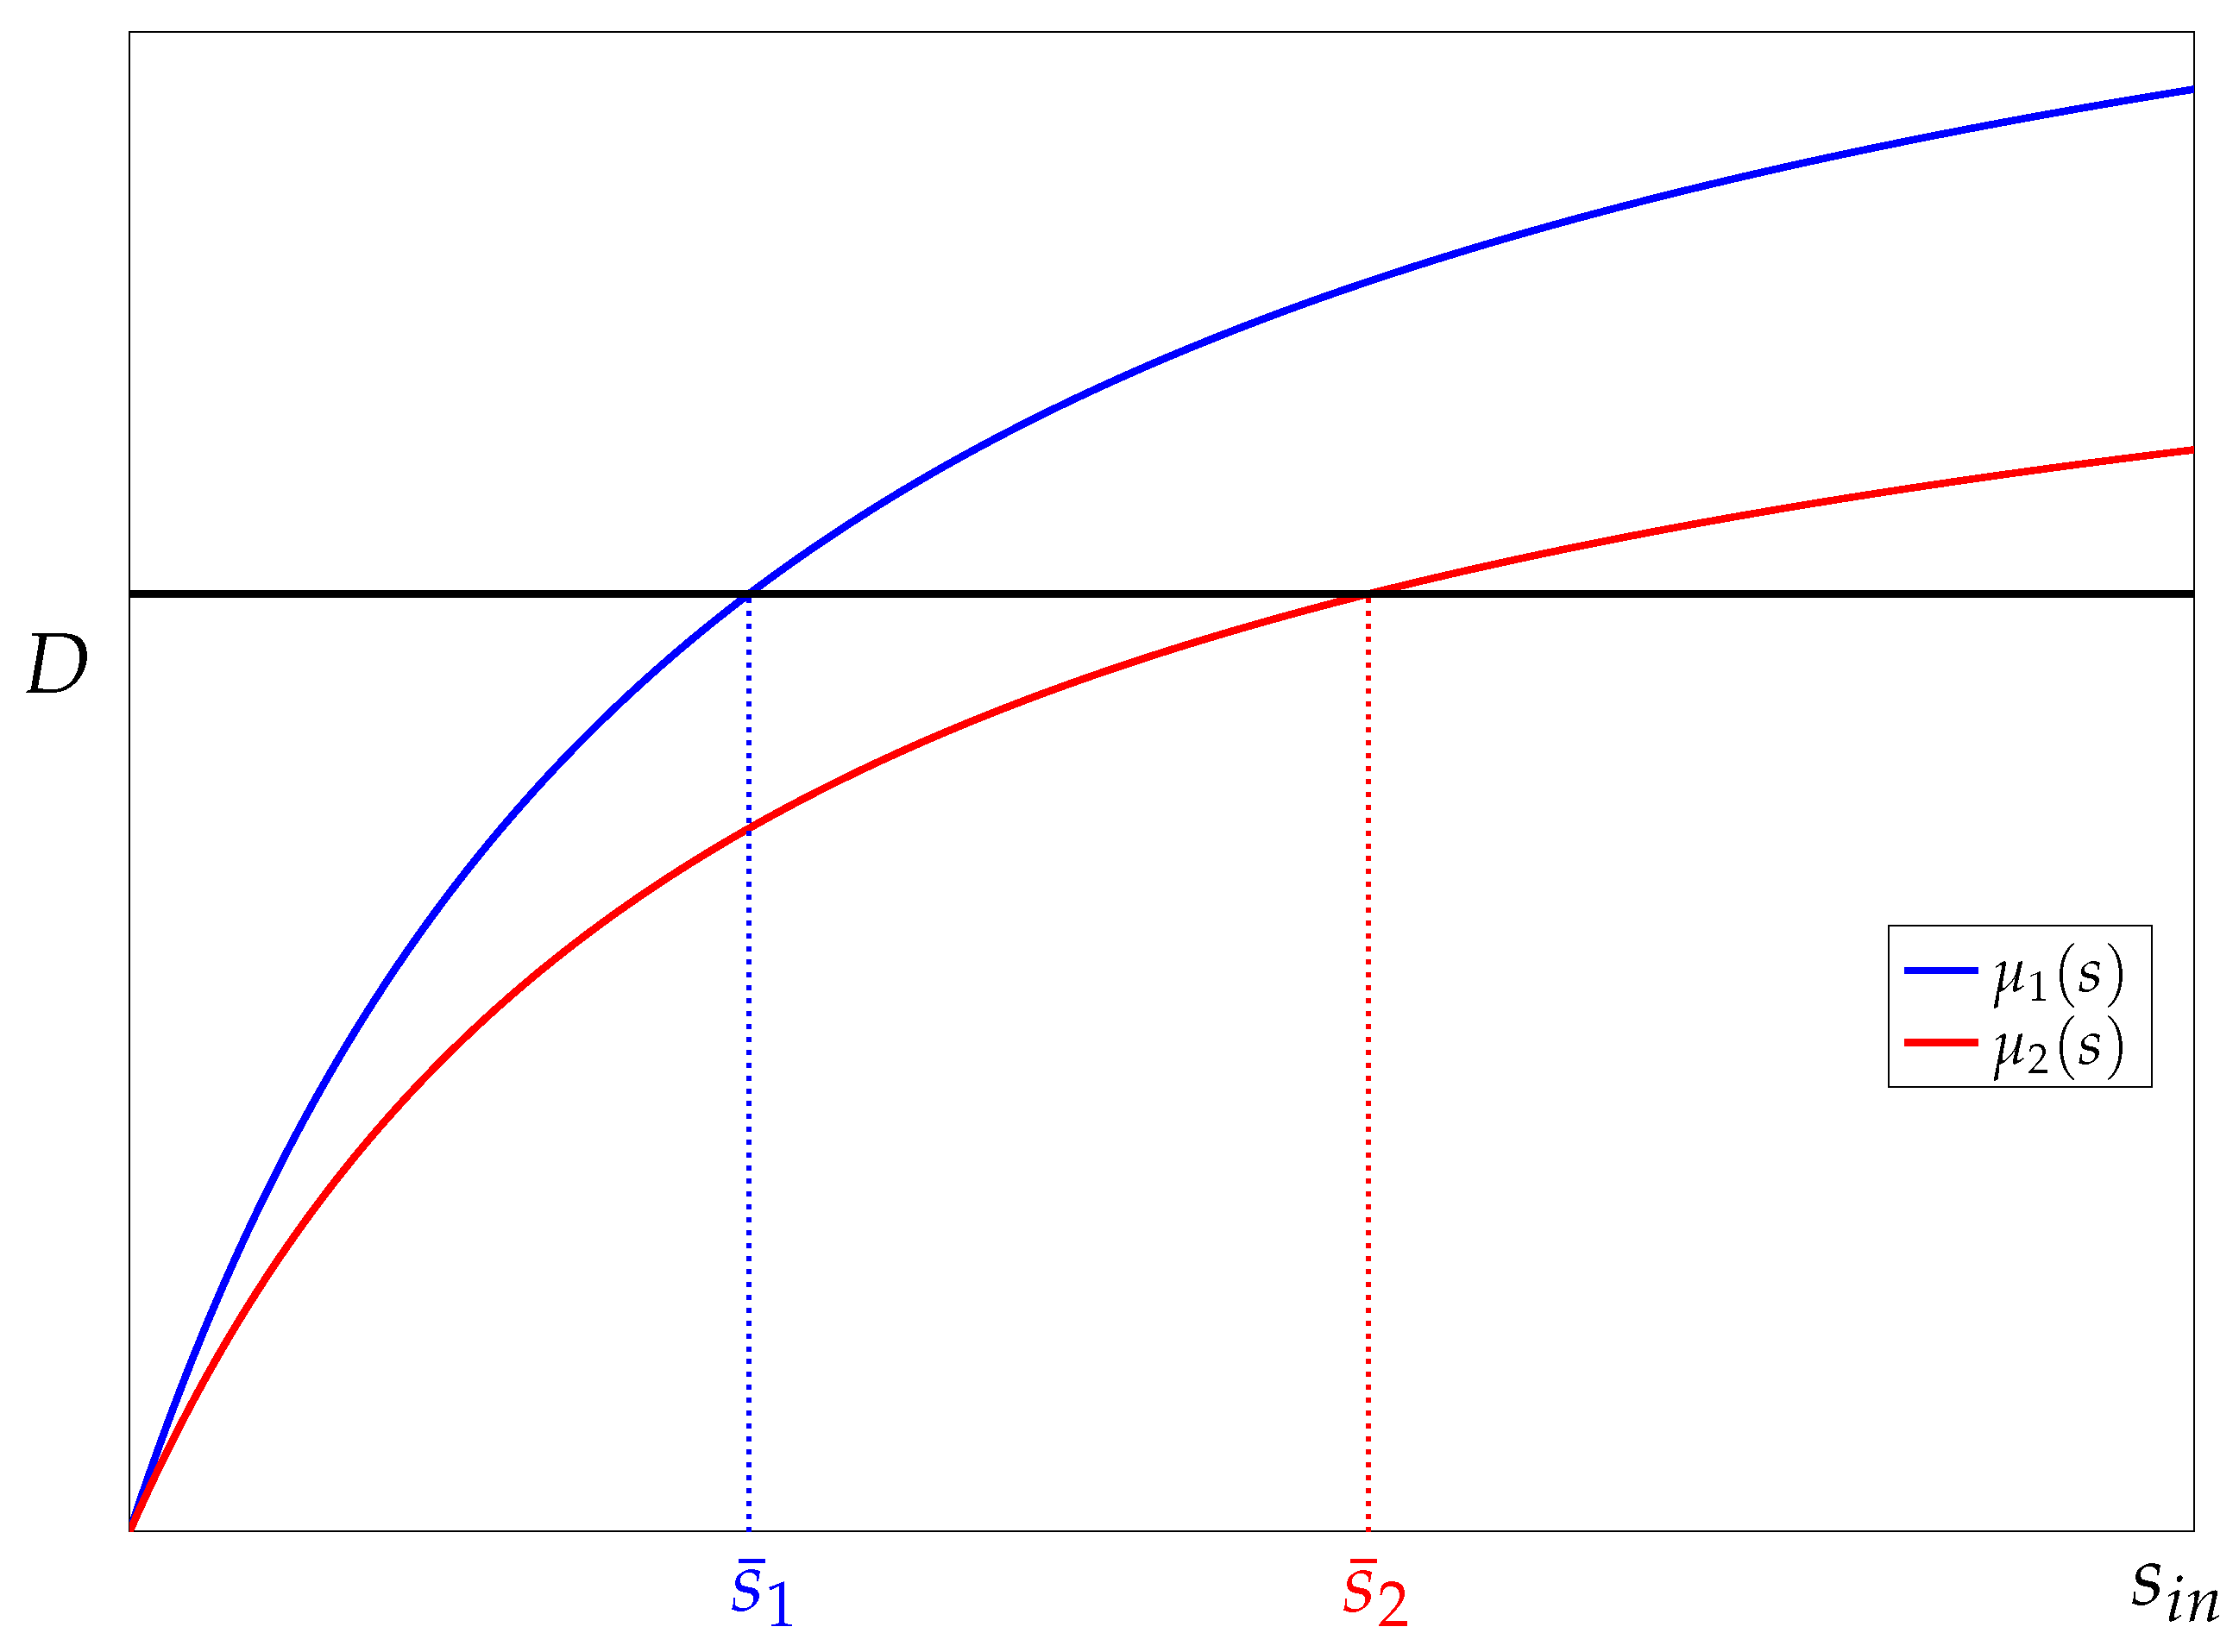
For the rest of the paper, assume that the growth rates and satisfy, as in Figure 3, the following assumption.
Figure 3.
Typical growth rates where .
Assumption A1.
and are increasing functions such that , and for all .
Under Assumption 1 and in order to define the equilibrium points, let the values and be the solutions of
and the solution of
and . Then, we have the following.
Lemma 1.
exist and are unique and satisfy .
Proof.
Since the functions and are continuous and increasing such that and , therefore exist and are unique. Let the function . Then , and . Therefore, the function f admits a unique root .
Since then . Since therefore . From the first equation of system (2) at a steady state where and , we deduce that satisfies with then then . Thus, we conclude that . □
2.2. Competition in the Absence of the Virus
Let consider the case of competition in the absence of the virus.
This model predicts (in the absence of the virus) the competitive exclusion, that is, at least one competitor species is extinct [29]. The species that has the best affinity with the substrate persists, and the other goes extinct. This principle was popularized by Hardin [30] and was mathematically investigated [2,21,22,31]. However, in real life, the coexistence of micro-organisms in bioreactors is widely noticed. Many mathematical modeling works were consecrated for explaining such a coexistence, either using the periodic input nutriment concentration [6,17], spatial considerations [32], or more recently using ratio-dependent growth rates [24,25].
Let , and be the three equilibrium points of the system (6) on the non-negative quadrant:
where according to Assumption 1. Then we obtain the following.
Proposition 2.
The steady state is globally asymptotically stable [29].
Let P be the “portion” in . We recall an alternative proof [33] of Proposition 2, providing the Lyapunov function. Let and the positively invariant set . Note that .
Proposition 3.
is globally asymptotically stable in Σ.
Proof.
Let the function
is a non-increasing function for all trajectories of the dynamics (6) in , where .
The derivative of the function along the solution of the dynamics (6) is
Since and satisfy Assumption 1, we have and for all . Then we obtain
Since , we obtain . Thus, is non-increasing along the solutions of system (6). Note that P is exactly the subset of where . By Lasalle’s invariance principle, we deduce that the trajectories converge inside the largest invariance set contained in P, which consists of the two steady states and . , which does not belong to but to its boundary, is a saddle point. We conclude that is globally asymptotically stable in . □
3. Steady States and Local Stability
We return to the main mathematical model (2) describing the competition of two species in a chemostat in the presence of a virus affecting only the first species. Let us define some operating parameters as follows: , , , , , , and . All the mentioned parameters are positive.
Furthermore, the following inequalities are useful for the rest of the paper.
Lemma 2.
and .
Proof.
Since and by Assumption 1, we obtain
Furthermore, we have and . □
For the equilibrium points, let us adopt the same notations given in [27]. Formally, let E, , , and be the five steady states of the system (2) on :
Note that E reflects the extinction of all species and the predator, reflects the extinction of the second species and the predator of the first species, while the first species is present. reflects the extinction of the first species and its predator, while the second species is present. reflects the coexistence of the first species and its predator, while the second species is extinct and, finally, reflects the coexistence of all species and the predator.
Then, one has the following results based on the linearization around the equilibria.
Lemma 3.
- 1.
- The trivial equilibrium point E exists, it is unique and it is always a saddle point.
- 2.
- exists, it is unique and it is always a saddle point.
- 3.
- exists, it is unique and it is a saddle point.
- 4.
- exists, it is unique and it is a saddle point.
- 5.
- exists, it is unique and it is locally asymptotically stable.
Proof.
See Appendix A. □
We sum up the above results as follows.
Theorem 1.
System (2) admits E, , , and as the equilibrium points. E, , and are saddle points and is a stable node.
4. Global Analysis
4.1. Reduction to 3D
Under Assumption 1, which ensures the existence of , the only stable steady state for the dynamics (2). E, , , and are saddle points. Solutions of the 4D dynamics (2) converge toward . Since our goal is to study the asymptotic behavior of these solutions, it is sufficient to restrict the study of the dynamics (2) onto the set . Therefore, by Thieme’s results [34], the asymptotic behavior of the trajectories will be informative for the complete dynamics (2); see [21,22] for other applications. The reduced dynamics of (2) on is
Thus, for (7) the state-vector belongs to the following subset of :
4.2. Periodic Orbits on the Faces
We start by excluding the possibility of periodic trajectory in one of the faces of the invariant set .
- Note that the axes and are invariant. Let us apply the transformation and for . Then, one obtains the following new system:
- Note that the axes and are invariant. Let us apply the transformation and for . Then one obtains the following new system:
- Note that the axes and are invariant. Let us apply the transformation and for . Then one obtains the following new system:
4.3. Persistence
In this section, we are interested in proving the coexistence of both species in terms of uniform persistence for the model (7). In our case, all boundary steady states of system (7) are unstable (saddle points). Therefore, we use the same prove as the one used in a similar situation in [35] by applying the Butler–McGehee Lemma [29] frequently. Hereafter, we recall a definition related to the uniform persistence [35] and the Butler–McGehee Lemma [29].
Definition 1.
Let us consider a system with where and . This system is weakly persistent if for every solution with a positive initial condition. It is persistent if for every solution with positive initial conditions. It is uniformly persistent if there exists a positive constant δ such that for every solution with a positive initial condition.
Lemma 4.
(Butler–McGehee Lemma [29]) Let be a continuously differentiable function. Let be a hyperbolic steady state of the system with . Let be the positive semi-orbit passing through and be the omega limit set of . Suppose that is inside , but is not the entire omega limit set. Therefore has a non-trivial intersection with both stable and unstable manifolds of .
Theorem 2.
The system (7) is persistent.
Proof.
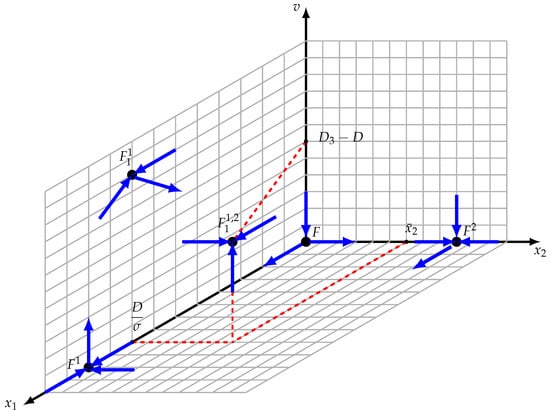
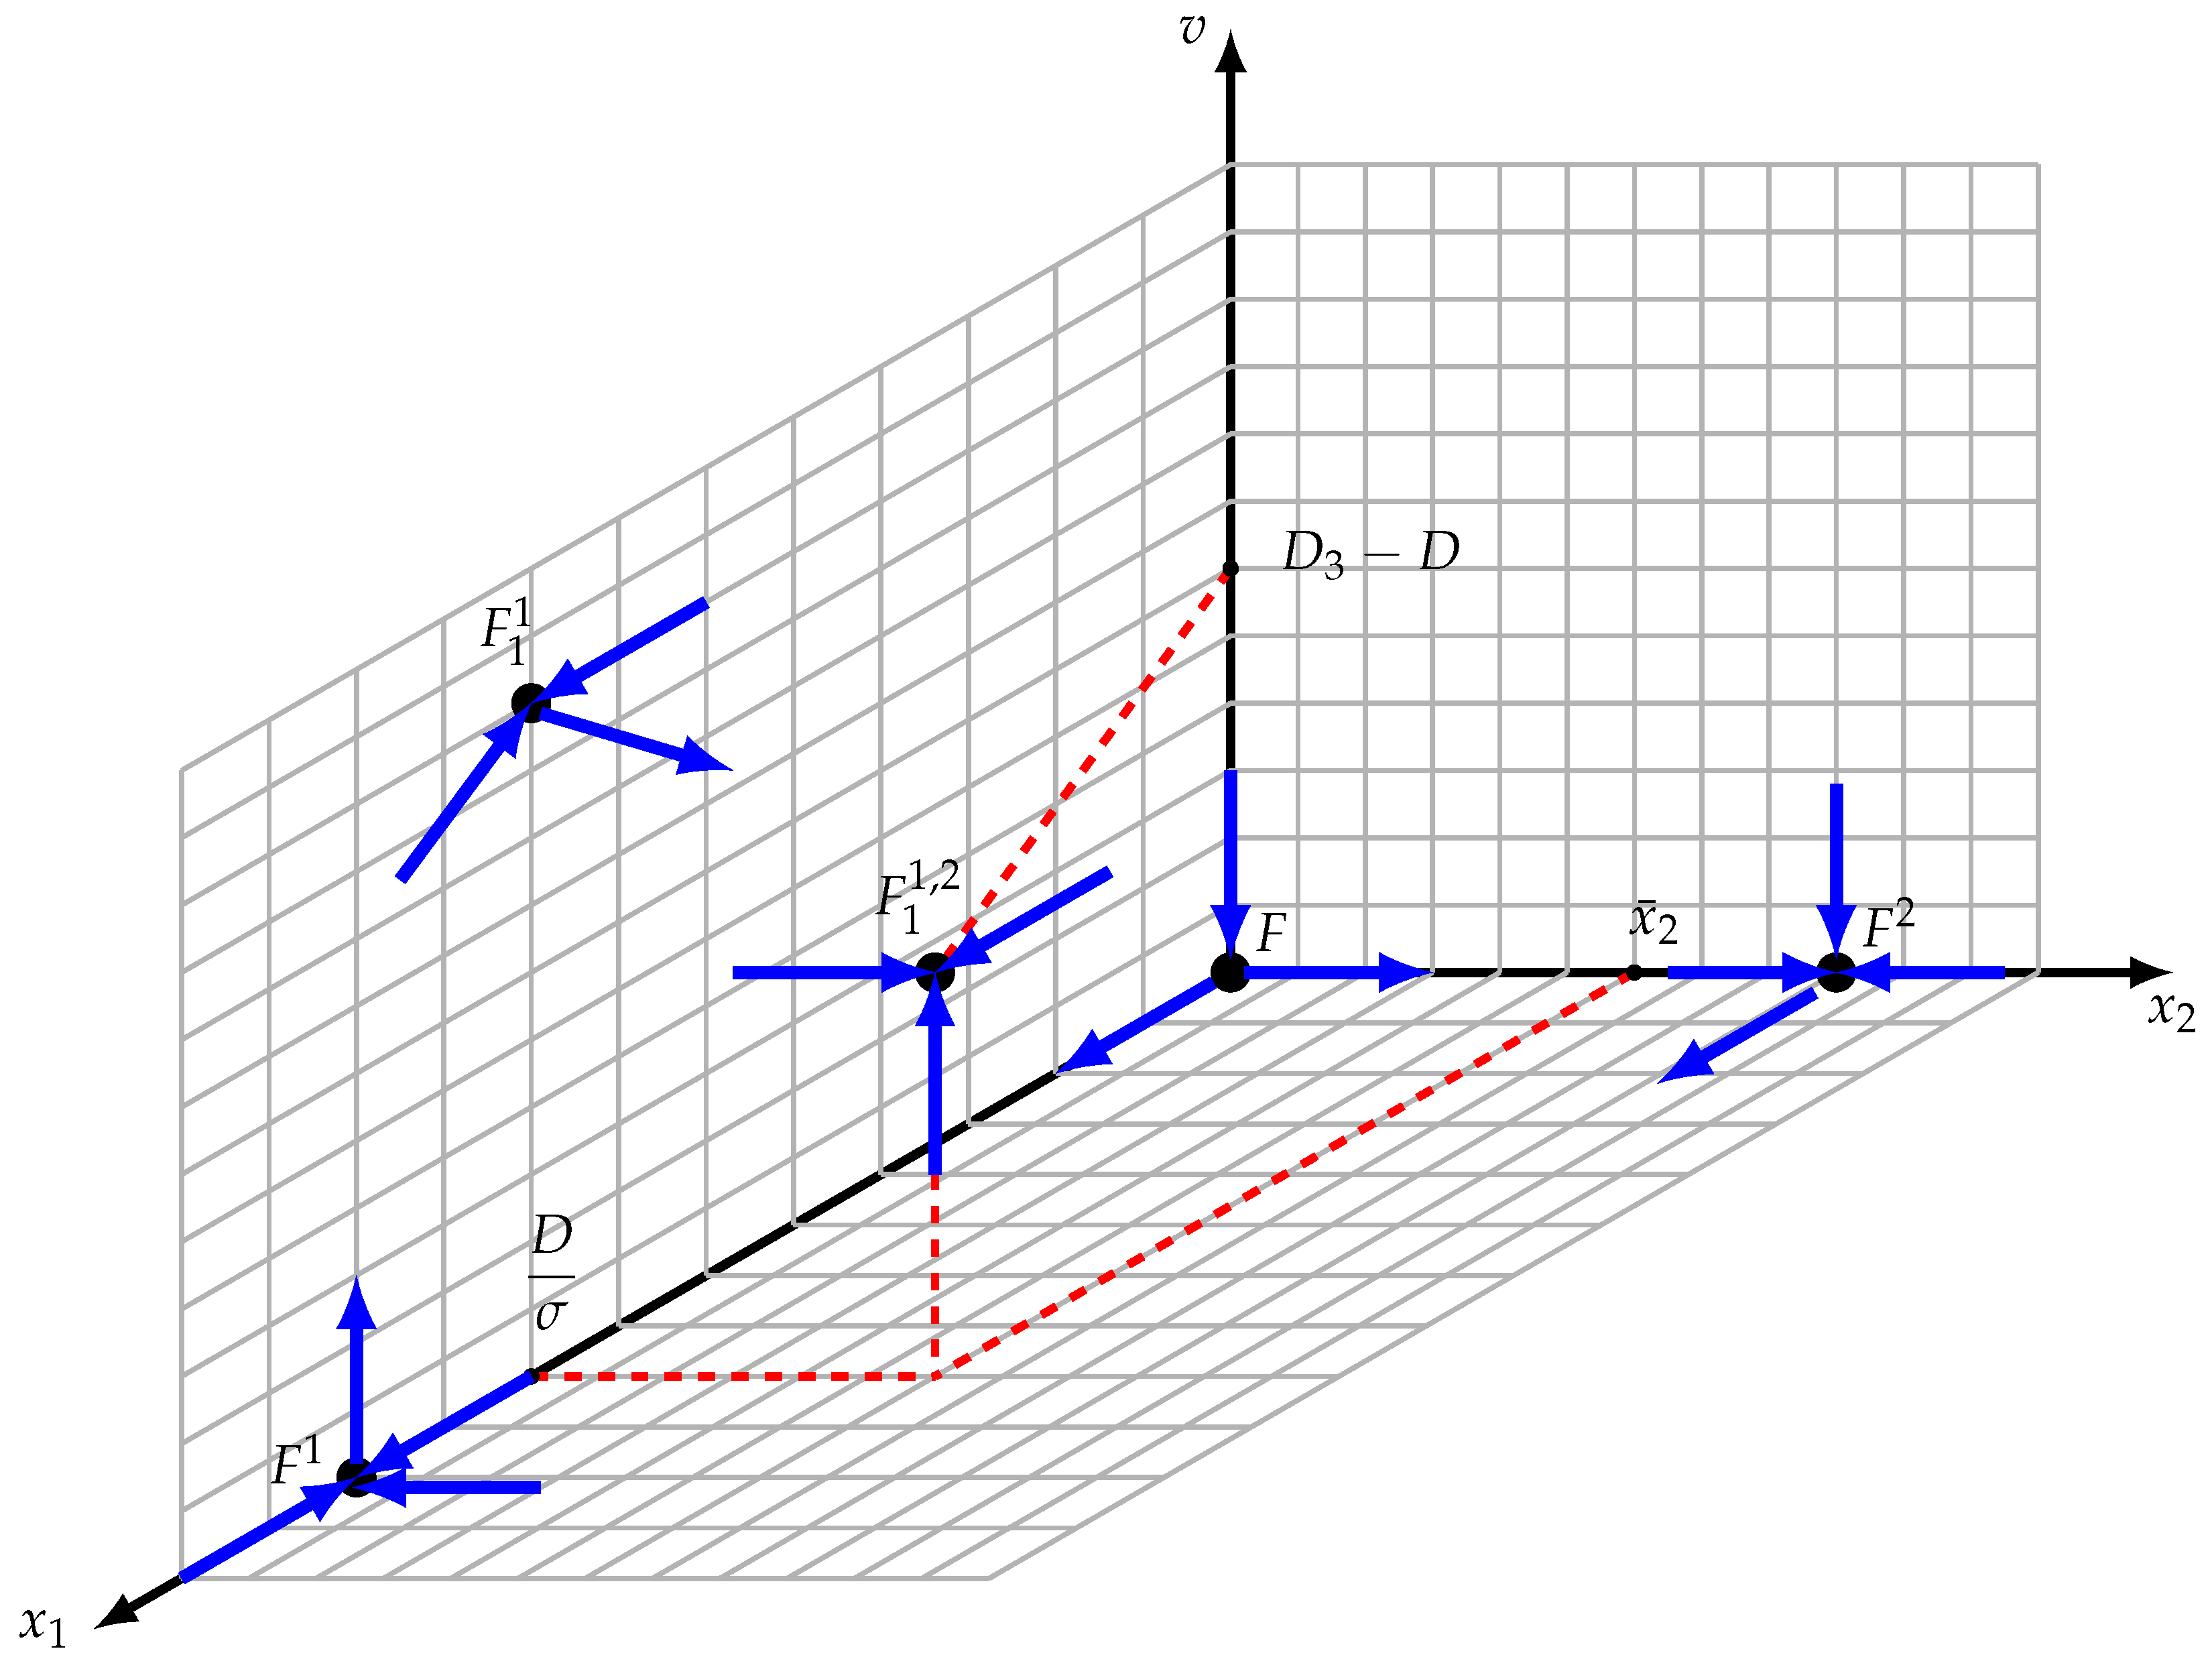
Since the three faces , , and are invariant, the stable and unstable manifolds of the boundary steady states are known and represented in Figure 4 to make the proof more clear. Consider a trajectory with initial trajectory where , and are given. We will prove by contradiction that the omega limit set has no point with a zero coordinate.
Figure 4.
Equilibria configuration. , and are saddle points; however, is an asymptotically stable interior equilibrium.
- Suppose that F is inside the omega limit set of denoted by . Note that F is a saddle point where its stable manifold is of dimension one and is restricted to the v-axis. Then F is not the entire omega limit set . Then, by the Butler–McGehee lemma [29], there exists a point in . Note that is the v-axis, but the v-axis is unbounded. Since all orbits of system (7) are bounded (inside the bounded set ), then the omega limit set of any orbit of (7) should be bounded. This contradicts the existence of . Then .
- Assume that . Since is a saddle point where its stable manifold is of dimension two and is restricted to the -plane. Then, is not the entire omega limit set . Thus, by the Butler–McGehee lemma [29], there exists a point inside . Since lies entirely in the -plane, and since the entire orbit through is in , this orbit is thus unbounded, which contradicts the fact that is inside .
- Assume that . By the same method as the cases of F and , we deduce that there exists a point inside . Here, the stable manifold is two-dimensional and lies entirely in the -face. Therefore, the entire orbit passing through which is inside becomes unbounded or its closure contains , which contradicts the fact that is inside .
- Assume that . Similarly, should not be the entire omega limit set ; therefore, there exists a point inside . This point should be inside the -face, once is 2-dimensional entirely contained in the -face. Similar to the cases of and , the entire orbit through should be inside . We proved previously in Section 4.2 that there are no possible periodic orbits inside the -face, and once , the orbit becomes unbounded, which contradicts the fact that is inside .
Now, let with at least one of the components , and be zero, and suppose that . Thus, the entire orbit passing through should be inside . However, since the orbit should lies entirely inside either , , or faces, it should converge to one of the boundary steady states since there is no possible periodic orbit. Thus, this boundary steady state is inside , which contradicts the fact that all boundary steady states are unstable. Therefore, each of the components of the trajectory is greater than zero, and then we proved that
and then the system (7) is persistent (see [35] (Section 4.3) for another application). □
4.4. Uniform Persistence of System (7)
Note that in several cases of biological models, persistence is equivalent to uniform persistence [36]. For our case, recall the result given in [36] affirming that if is a dynamical system such that and are both invariant. Let be the restriction of to . Therefore, is uniformly persistent under some conditions given hereafter
- is weakly persistent;
- is dissipative (i.e., and the closure of is compact);
- is isolated;
- is acyclic.
Let be the dynamics on defined in Proposition 1. is not invariant; however, the theorem in [36], as applied in [35,37], should be applied when and is invariant on but repelling into the interior of on , provided that both conditions 3 and 4 are verified when restricting to . For our system, the invariant set is bounded. Thus, condition 1 is satisfied. Since the persistence implies the weak persistence, condition 2 holds by Theorem 2. Furthermore, condition 3 is verified since all boundary steady states are hyperbolic, so every one of them is the maximal invariant set in its neighborhood, and furthermore, the union of the steady states forms a covering of the omega limit sets of . Condition 4 is also verified since the boundary steady states are not linked cyclically. Therefore, we deduce the uniform persistence of system (7) as mentioned in the following theorem.
Theorem 3.
The system (7) is uniformly persistent, i.e., there exists a constant , independent of the initial condition, with
4.5. Uniform Persistence of System (2)
Let us now extend the persistence result to prove that the main system (2) is uniformly persistent. Note that if with and , then we should have . However, there exist and a time sequence () that converges to ∞, where the associated trajectory converges to . This implies that is not globally attracting, which contradicts the proposition 1. Furthermore, assume that contains a point on a boundary face, where one of the variable or v is zero; therefore, the entire orbit passing through this point should be inside . Therefore, the omega limit set is entirely contained inside . Therefore, we deduce the main result hereafter.
Theorem 4.
The system (2) is uniformly persistent.
5. Numerical Simulations
We perform numerical results on a system that uses Monod functions to express growth rates:
where and are constants. One can readily check that the functions and satisfy Assumption 1. Consider the parameters values given in the following Table 1.
Table 1.
The chosen parameters in the numerical simulations are used to just illustrate the results, and they have no practical biological significance.
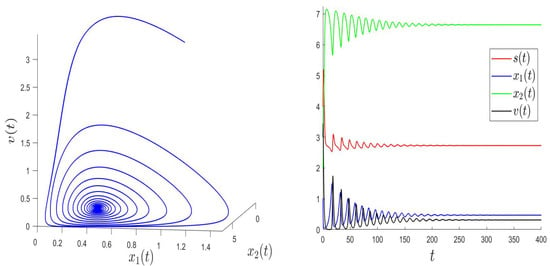
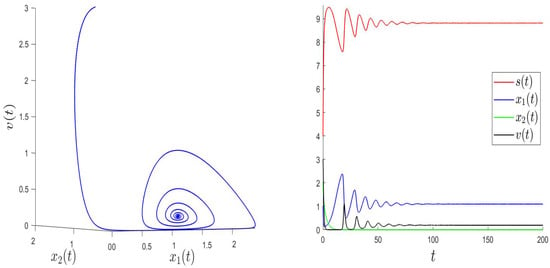
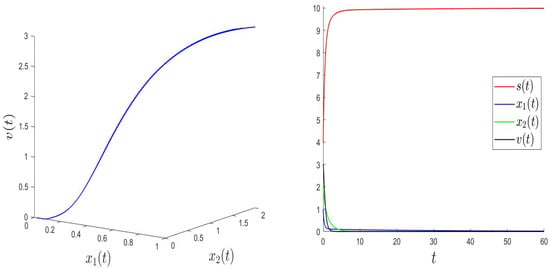
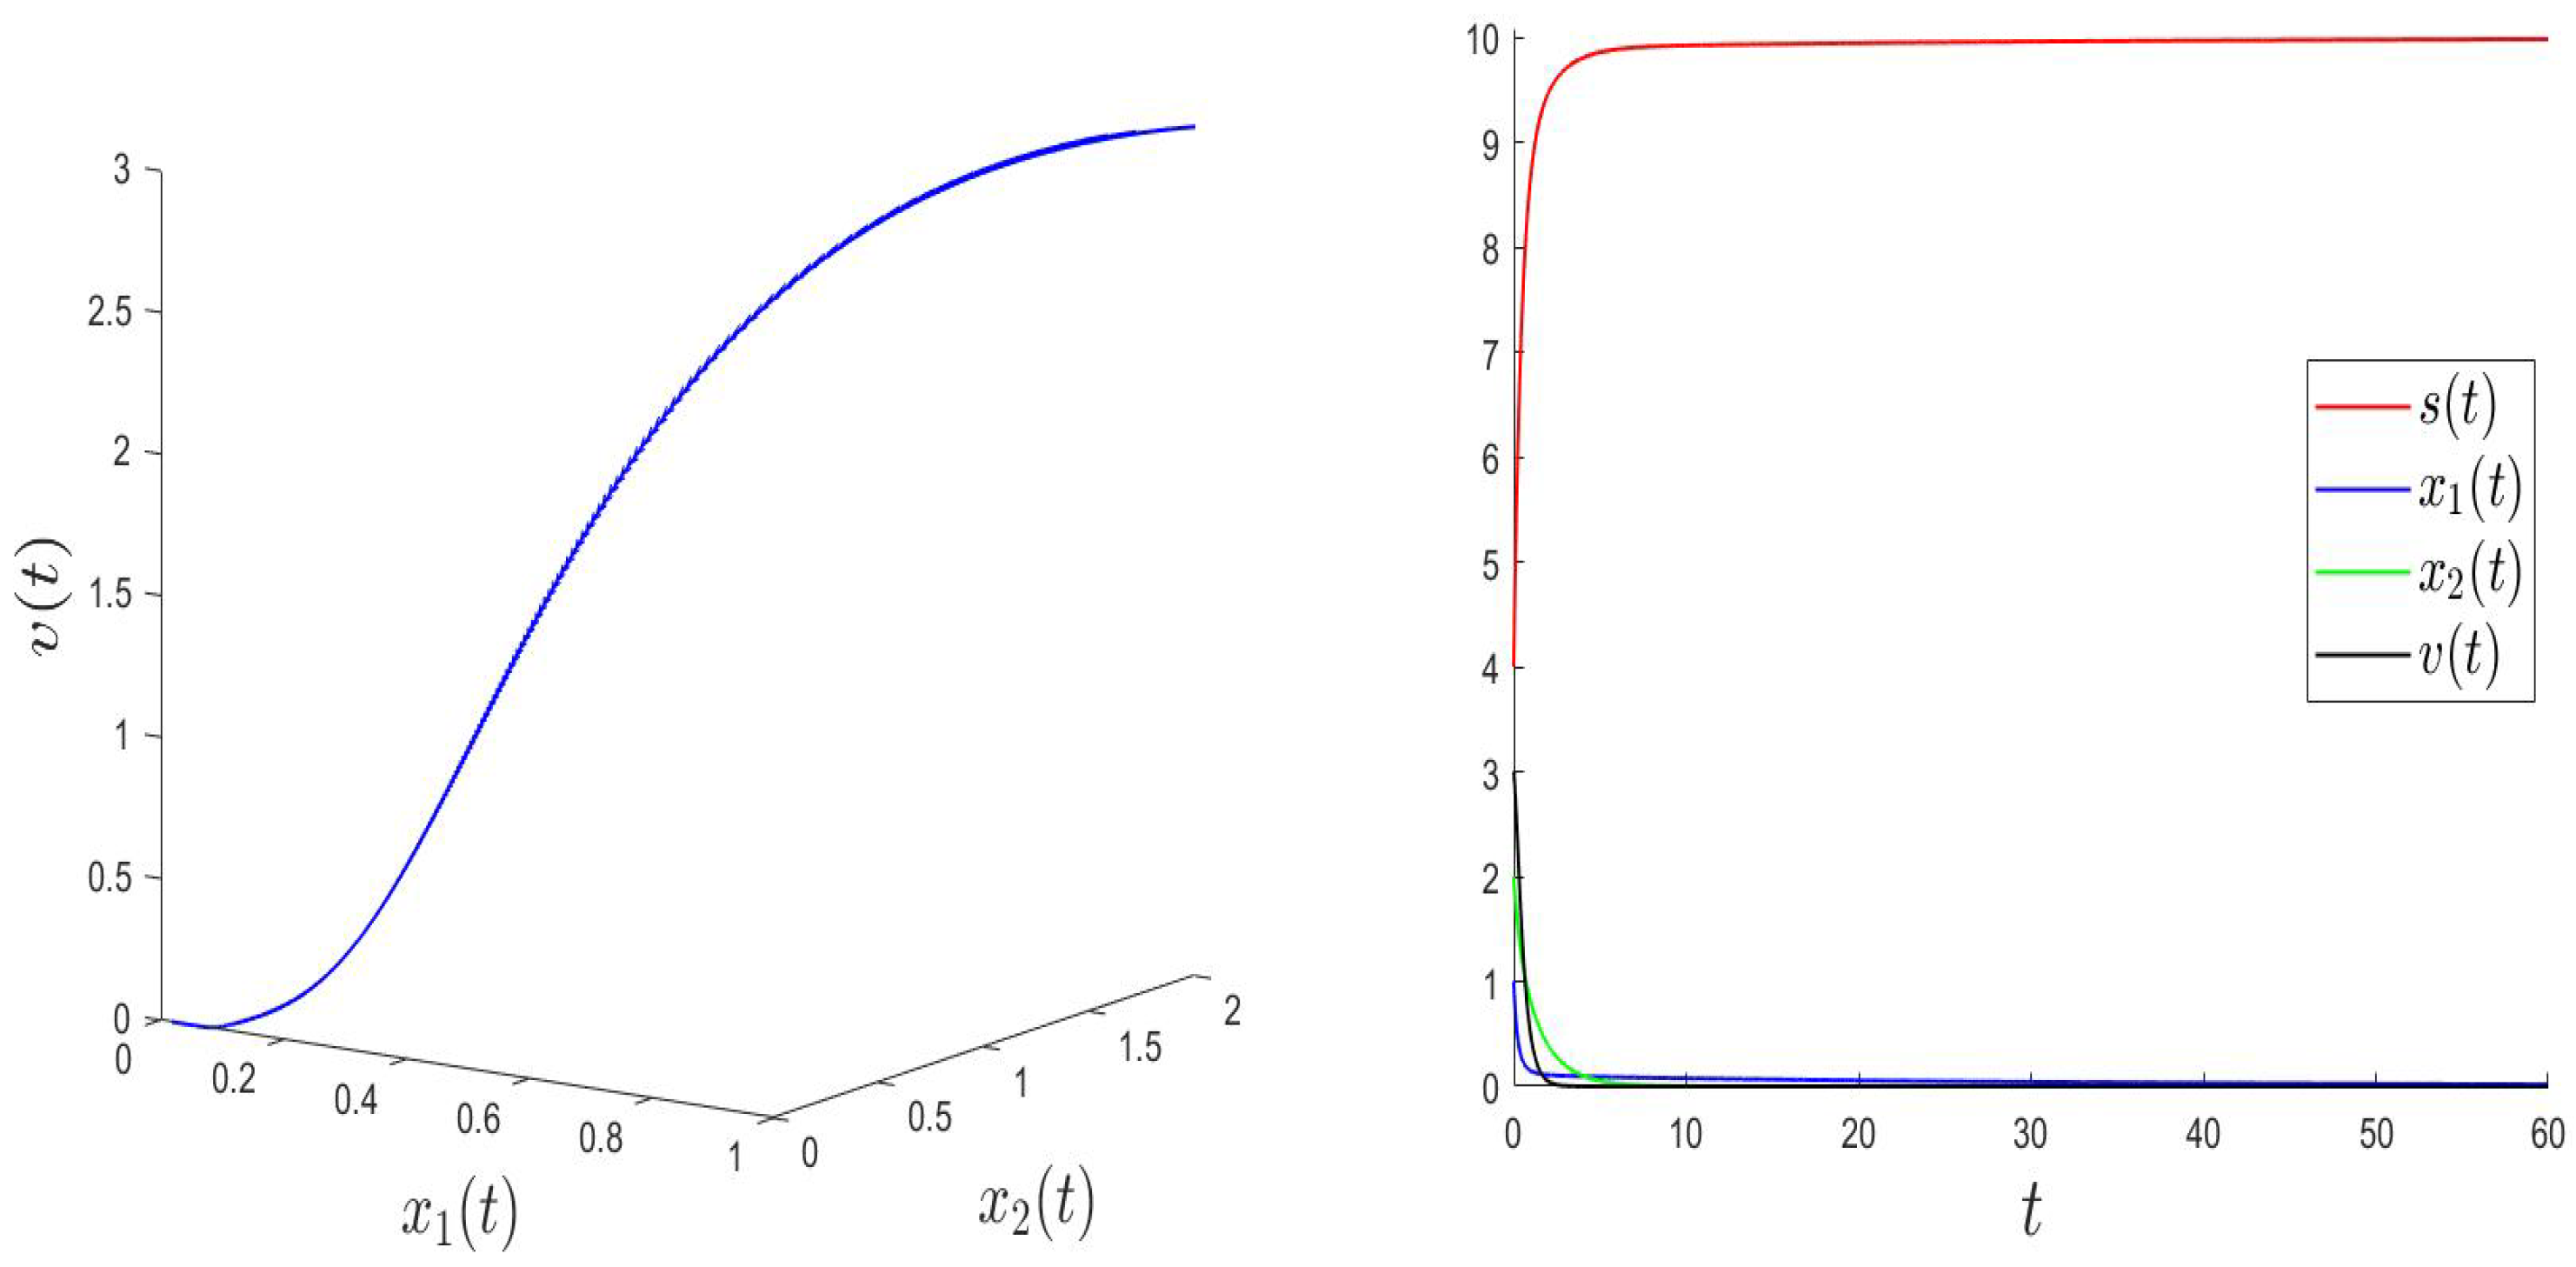
We give some numerical results confirming the theoretical findings in Figure 5, Figure 6 and Figure 7. In Figure 5, the solution of the system (2) converges to the equilibrium , where the two species coexist, contradicting the competitive exclusion principle which affirms that at most, one species of micro-organisms is able to survive long term, while the other species should disappear. In Figure 6, the solution of the system (2) converges to the equilibrium , where only species 1 persists with the virus, which confirms the competitive exclusion principle. Finally, in Figure 7, the solution of the system (2) converges to the equilibrium E, where the two species go extinct. Note that the numerical simulations given in Figure 6 and Figure 7 illustrate that there is no coexistence of both species (species and species ) without the presence of the virus (v) and the satisfaction of Assumption 1, where . This situation contradicts the competitive exclusion principle, which affirms that in such a competition, at most, one species can avoid extinction.
Figure 5.
, , , , , , , , , . Assumption 1 is satisfied, and the solution of the system (2) converges to the positive equilibrium , where the two species coexist.
Figure 6.
, , , , , , , , . Assumption 1 is not satisfied, and the solution of the system (2) converges to the equilibrium , where only species 1 persists with the virus.
Figure 7.
, , , , , , . Assumption 1 is not satisfied, and the solution of the system (2) converges to the equilibrium E, where the two species goes extinct.
6. Conclusions
The competitive exclusion principle is valid for purely exploitative competition for a single resource, and once you allow additional mechanisms of competition, as it is in this paper, coexistence becomes possible. It would be interesting and theoretically significant to investigate the possibility of virus-mediated coexistence: when the species cannot coexist unless the viruses are present. We considered a competition of two micro-organisms for a single essential growth-limiting nutriment in the presence of a virus that affects only the first species. We proposed a four-dimensional system of differential equations. By neglecting all possible decay terms, we reduced the system to a three-dimensional one. Then, since all boundary steady states of our system are unstable, we applied the Butler–McGehee Lemma [29] frequently, which helped us to apply the theory of uniform persistence [35] to prove the coexistence of the two competing species and the virus. We proved that there is no coexistence of both species without the presence of the virus and the satisfaction of some assumptions on the growth rates of species. We confirmed the theoretical results by some numerical simulations.
Author Contributions
Conceptualization, M.E.H. and A.A.A.; Methodology, M.E.H. and A.A.A.; Writing—original draft, M.E.H. and A.A.A.; Writing—review and editing, M.E.H. and A.A.A. All authors have read and agreed to the published version of the manuscript.
Funding
This project was funded by the Deanship of Scientific Research (DSR) at King Abdulaziz University, Jeddah, Saudi Arabia under grant no. (G: 546-130-1443).
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
Not applicable.
Acknowledgments
This project was funded by the Deanship of Scientific Research (DSR) at King Abdulaziz University, Jeddah, Saudi Arabia under grant no. (G: 546-130-1443). The authors, therefore, acknowledge with thanks DSR for the technical and financial support. The authors are also grateful to the unknown referees for the many constructive suggestions, which helped to improve the presentation of the paper.
Conflicts of Interest
The authors declare no conflict of interest.
Appendix A. Proof of Lemma 3
Proof.
The Jacobian linearization matrix of dynamics (2) at a point is then given by
- Its eigenvalues are given by and . Therefore, E is a saddle point.
- The Jacobian linearization matrix of dynamics (2) at the point is then given byThe characteristic polynomial is given byIts eigenvalues are given by and . Therefore, is a saddle point.
- The Jacobian linearization matrix of dynamics (2) at the point is then given byThe characteristic polynomial is given byIts eigenvalues are given by and . Therefore, is a saddle point.
- The Jacobian linearization matrix of dynamics (2) at the point is then given byThe characteristic polynomial is given byThe first two eigenvalues are given by . The other two eigenvalues are the solution ofSince and then these two eigenvalues are of negative real parts. Therefore, is a saddle point.
- The Jacobian linearization matrix of dynamics (2) at the point is then given byThe characteristic polynomial is given bywhereThe conditions of stability are written as the following:Since we havethen the equilibrium point is always locally asymptotically stable.
□
References
- Hsu, S.B.; Hubbell, S.; Waltman, P. A mathematical theory for single-nutrient competition in continuous cultures of micro-organisms. SIAM J. Appl. Math. 1977, 32, 366–383. [Google Scholar] [CrossRef] [Scilit]
- Butler, G.J.; Wolkowicz, G.S.K. A mathematical model of the chemostat with a general class of functions describing nutrient uptake. SIAM J. Appl. Math. 1985, 45, 138–151. [Google Scholar] [CrossRef] [Scilit]
- Wolkowicz, G.S.K.; Lu, Z. Global dynamics of a mathematical model of competition in the chemostat: General response functions and differential death rates. SIAM J. Appl. Math. 1992, 52, 222–233. [Google Scholar] [CrossRef] [Scilit]
- Smith, H.L.; Waltman, P. Competition for a single limiting resource in continuous culture: The variable-yield model. SIAM J. Appl. Math. 1994, 54, 1113–1131. [Google Scholar] [CrossRef] [Scilit]
- Hsu, S.B. A competition model for a seasonally fluctuating nutrient. J. Math. Biol. 1980, 9, 115–132. [Google Scholar] [CrossRef] [Scilit]
- Smith, H.L. Competitive coexistence in an oscillating chemostat. SIAM J. Appl. Math. 1981, 40, 498–522. [Google Scholar] [CrossRef] [Scilit]
- Hale, J.K.; Somolinos, A.S. Competition for a fluctuating nutrient. J. Math. Biol. 1983, 18, 255–280. [Google Scholar] [CrossRef] [Scilit]
- Smith, H.L.; Thieme, H.R. Chemostats and epidemics: Competition for nutrients/hosts. Math. Biosci. Eng. 2013, 10, 1635–1650. [Google Scholar]
- Korytowski, D.; Smith, H. Permanence and Stability of a Kill the Winner Model in Marine Ecology. Bull. Math. Biol. 2017, 79, 995–1004. [Google Scholar] [CrossRef] [Scilit]
- Browne, C.; Smith, H. Dynamics of virus and immune response in multi-epitope network. J. Math. Biol. 2018, 77, 1833–1870. [Google Scholar] [CrossRef] [Scilit]
- Wade, M.; Harmand, J.; Benyahia, B.; Bouchez, T.; Chaillou, S.; Cloez, B.; Godon, J.J.; Boudjemaa, B.M.; Rapaport, A.; Sari, T.; et al. Perspectives in mathematical modelling for microbial ecology. Ecol. Model. 2016, 321, 64–74. [Google Scholar] [CrossRef] [Scilit]
- Vandermeer, J.; Pascual, M. Competitive coexistence through intermediate polyphagy. Ecol. Complex. 2006, 3, 37–43. [Google Scholar] [CrossRef] [Scilit]
- El Hajji, M.; Mazenc, F.; Harmand, J. A mathematical study of a syntrophic relationship of a model of anaerobic digestion process. Math. Biosci. Eng. 2010, 7, 641–656. [Google Scholar] [PubMed]
- Sari, T.; El Hajji, M.; Harmand, J. The mathematical analysis of a syntrophic relationship between two microbial species in a chemostat. Math. Biosci. Eng. 2012, 9, 627–645. [Google Scholar] [PubMed]
- Albargi, A.H.; El Hajji, M. Mathematical analysis of a two-tiered microbial food-web model for the anaerobic digestion process. Math. Biosci. Eng. 2023, 20, 6591–6611. [Google Scholar] [CrossRef] [Scilit]
- Stephanopoulos, G.; Fredrickson, A.; Aris, R. The growth of competing microbial populations in a CSTR with periodically varying inputs. AIChE J. 1979, 25, 863–872. [Google Scholar] [CrossRef] [Scilit]
- Butler, G.J.; Hsu, S.B.; Waltman, P. A mathematical model of the chemostat with periodic washout rate. SIAM J. Appl. Math. 1985, 45, 435–449. [Google Scholar] [CrossRef] [Scilit]
- Zhao, X. Dynamical Systems in Population Biology; Springer: New York, NY, USA, 2003; Volume 16. [Google Scholar]
- Hsu, S.B.; Waltman, P. Analysis of a model of two competitors in a chemostat with an external inhibitor. SIAM J. Appl. Math. 1991, 52, 528–540. [Google Scholar] [CrossRef] [Scilit]
- Ballyk, M.; Wolkowicz, G.S.K. Exploitative competition in the chemostat for two perfectly substitutable resources. Math. Biosci. 1993, 118, 127–180. [Google Scholar] [CrossRef] [Scilit]
- El Hajji, M.; Harmand, J.; Chaker, H.; Lobry, C. Association between competition and obligate mutualism in a chemostat. J. Biol. Dyn. 2009, 3, 635–647. [Google Scholar] [CrossRef] [Scilit]
- El Hajji, M. How can inter-specific interferences explain coexistence or confirm the competitive exclusion principle in a chemostat. Int. J. Biomath. 2018, 11, 1850111. [Google Scholar] [CrossRef] [Scilit]
- Grognard, F.; Mazenc, F.; Rapaport, A. Polytopic Lyapunov functions for the stability analysis of persistence of competing species. In Proceedings of the 44th IEEE Conference on Decision and Control and European Control Conference, Seville, Spain, 12–15 December 2005. [Google Scholar]
- Lobry, C.; Mazenc, F.; Rapaport, A. Persistence in ecological models of competition for a single resource. C.R. Acad. Sci. Paris, Ser I 2004, 340, 199–240. [Google Scholar] [CrossRef] [Scilit]
- Lobry, C.; Harmand, J. A new hypothesis to explain the coexistence of n species in the presence of a single resource. Comptes Rendus Biol. 2006, 329, 40–46. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mazenc, F.; Lobry, C.; Rapaport, A. Persistence in Ratio-Dependent Models of Consumer-Resource Dynamics. Electron. J. Differ. Equations (EJDE) 2007, 2007, 211–220. [Google Scholar]
- Wolkowicz, G.S. Successful invasion of a food web in a chemostat. Math. Biosci. 1989, 93, 249–268. [Google Scholar] [CrossRef] [Scilit]
- Steiner, C.; Klausmeier, C.; Litchman, E. Transient dynamics and the destabilizing effects of prey heterogeneity. Ecology 2012, 93, 632–644. [Google Scholar] [CrossRef] [Scilit]
- Smith, H.L.; Waltman, P. The Theory of the Chemostat. Dynamics of Microbial Competition; Cambridge Studies in Mathematical Biology, Cambridge University Press: Cambridge, UK, 1995; Volume 13. [Google Scholar]
- Hardin, G. The competition exclusion principle. Science 1960, 131, 1292–1298. [Google Scholar] [CrossRef] [Scilit]
- Aris, R.; Humphrey, A.E. Dynamics of a chemostat in which two organisms compete for a common substrate. Biotechnol. Bioeng. 1977, 19, 1375–1386. [Google Scholar] [CrossRef] [Scilit]
- Stephanopoulos, G.; Fredrickson, A.G. Effect of inhomogeneities on the coexistence of competing microbial populations. Biotechnol. Bioeng. 1979, 21, 1491–1498. [Google Scholar] [CrossRef] [Scilit]
- El Hajji, M.; Rapaport, A. Practical coexistence of two species in the chemostat - A slow-fast characterization. Math. Biosci. 2009, 218, 33–39. [Google Scholar] [CrossRef] [Scilit]
- Thieme, H.R. Convergence results and a Poincaré-Bendixson trichotomy for asymptotically autonomous differential equations. J. Math. Biol. 1992, 30, 755–763. [Google Scholar] [CrossRef] [Scilit]
- Sobieszek, S.; Wade, M.J.; Wolkowicz, G.S.K. Rich dynamics of a three-tiered anaerobic food-web in a chemostat with multiple substrate inflow. Math. Biosci. Eng. 2020, 17, 7045–7073. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Butler, G.J.; Freedman, H.I.; Waltman, P. Uniformly persistent systems. Proc. Am. Math. Soc. 1986, 96, 425–429. [Google Scholar] [CrossRef]
- Butler, G.; Wolkowicz, G. mediated coexistence in a chemostat: Coexistence and competition reversal. Math. Model. 1987, 8, 781–785. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2023 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).