


Abstract
Nowadays, Cannabis sativa L. is primarily valued for the cannabinoids produced and accumulated in its glandular trichomes. Consequently, it is of special relevance to address studies related to the biochemical, molecular, and morphological panorama of trichomes. This review highlights some of the most recent publications on the morphological, phenological, biochemical and molecular characterization of trichomes and mechanisms underlying their development. Particular emphasis is placed on the transcription factors related to trichome cell identity, drawing on studies conducted in model organisms and in Cannabis sativa L. Finally, we discuss emerging approaches for studying trichomes and highlight biotechnological perspectives that may facilitate future research and crop improvement.
1. Introduction
Cannabis sativa L. (thereafter Cannabis) [1] is an annual, herbaceous, predominantly outcrossing species indigenous to the Tibetan Plateau [2,3]. Cannabis plant life cycle comprises four discrete developmental phases: germination and seedling establishment, vegetative growth, flowering and seed formation [4]. Cannabis pistillate flowers are characterized by a reduced perianth and a well-developed perigonal bract that encloses the ovary and the two stigmas. On the epidermis of the bract, specialized structures called trichomes accumulate, displaying high density and heterogeneous morphologies.
Trichomes perform key functions including secondary metabolite synthesis and storage, defense against herbivory, UV protection and water regulation [5,6]. Whereas species like Arabidopsis thaliana produce only unicellular, non-glandular (typically branched) trichomes [7], other species including Artemisia annua and Solanum lycopersicum display a plethora of trichome morphologies generally classified as non-glandular or as glandular trichomes. Glandular trichomes mediate the synthesis and accumulation of metabolites such as acyl sugars, terpenoids, flavonoids, artemisinin, among others [8,9].
As depicted in Figure 1, the Cannabis plant presents glandular and non-glandular trichomes [10]. Non-glandular trichomes accumulate silica (SiO2·nH2O) and are further classified as cystolithic or non-cystolithic depending on the presence or absence of a calcium carbonate (CaCO3) cystolith. Cystolithic trichomes present conical shapes and reach ~150 μm in height, whereas non-cystolithic trichomes are more elongated and tapering, extending up to ~400 μm. Both types are considered part of the plant’s physical and mechanical defense system [11].
Figure 1.
Trichome types on Cannabis epidermis. Microscope photograph of Cannabis female bract surface showing different trichome types (A). Trichome types representation (B). Glandular trichomes: capitate-stalked, capitate sessile and bulbous glandular trichomes. Non-glandular trichomes: cystolithic and hair-like trichomes. Created in https://BioRender.com.
Cannabis glandular trichomes are characterized by having a subcuticular storage cavity in their most distal region, where specialized metabolites accumulate. The size of this cavity distinguishes three subtypes: bulbous, sessile and capitate-stalked (Figure 1B). Bulbous trichomes have fewer cells, consisting of one to two cells in the stem and four in the globular head; therefore, they are the smallest trichomes with a diameter ranging between 10 μm and 20 μm. Sessile glandular trichomes possess a larger-diameter globular structure (>30 μm), and although defined as sessile, they show a small stalk of one cell in height and four cells in width [11]. Capitate-stalked glandular trichomes (CSGTs) show a clearly defined stalk and globular head of larger diameter. This type of trichome shows the largest dimensions; however, its phenotype is not homogeneous, and contrasting and intermediate morphologies are observed [11,12]. Glandular trichomes are usually present in flower tissue of female inflorescences. Monoecious and male plants also develop these structures, although in a lower density [13,14,15].
The specialized metabolites of greatest biomedical and commercial interest in Cannabis are cannabinoids, a group of terpenophenolic compounds that accumulate in the heads of glandular trichomes. Cannabinoids have applications in the medicinal, cosmetic, and recreational industries, which have contributed to their commercial value following legalization in various countries [5,16]. Cannabigerolic acid (CBGA) is the common precursor of the major cannabinoids tetrahydrocannabinolic acid (THCA) and cannabidiolic acid (CBDA), which are subsequently decarboxylated to Δ9-tetrahydrocannabinol (D9-THC) and cannabidiol (CBD), respectively [17].
Currently, Arabidopsis thaliana remains the best-studied genetic model for regulation of non-glandular trichome morphogenesis. Over the past decades, studies in Arabidopsis have defined a core regulatory logic centered on transcription factor complexes that promote cell identity [18,19,20], downstream factors that support differentiation [21,22], and mobile repressors that refine epidermal spacing through lateral inhibition [23]. Although this framework was established in a non-glandular context, it offers a valuable conceptual foundation for comparative studies, as it highlights recurrent regulatory principles that may also operate in glandular trichome formation and function in other species.
Converging evidence across plant lineages indicates that regulatory modules involving R2R3-MYB, bHLH, and HD-ZIP IV factors have important roles as regulators of trichome morphogenesis and specialized metabolism [24,25,26]. Studies addressing spatiotemporal expression and interaction between these genes will be essential to explain traits such as glandular trichome density in flowers and leaves, with the intention of looking for increases in cannabinoid accumulation yields. Identification of these genes has the potential to accelerate targeted metabolic enhancement and therefore precision plant breeding of Cannabis [27].
This review synthesizes current knowledge on the morphology and genetic regulation of glandular trichome development in Cannabis. Additionally, we briefly survey functional tools that enable hypothesis-driven analysis of gene regulation and protein interaction in the context of trichome development. Because direct functional evidence on the genetic regulation of glandular trichome development in Cannabis remains limited, we provide an extensive comparative analysis of well-characterized model species, particularly Arabidopsis thaliana, Solanum lycopersicum, and Artemisia annua.
The literature search strategy for this review was based on searches of Google Scholar using combinations of keywords related to glandular trichome development, transcriptional regulation, specialized metabolism, and Cannabis, together with searches focused on Arabidopsis thaliana, Solanum lycopersicum, and Artemisia annua. Most publications considered were published between 2015 and 2026, with emphasis on original studies providing genetic, transcriptomic, molecular, biochemical, or functional evidence related to trichome development and specialized metabolism. Earlier publications were also included when they provided foundational evidence or were identified as relevant references in the selected literature.
Herein, we propose a theoretical framework underlying trichome development, informed by insights from established plant models. Given the ongoing debate regarding the taxonomy of Cannabis, throughout this review we used Cannabis rather than Cannabis sativa and/or indica and/or variety indica or sativa [28].
2. Structure and Development of Capitate-Stalked Glandular Trichomes in Cannabis
CSGT structure features a group of six cells that transversally divide to form a stalk with seven to ten cells and a combined length ranging from 20 μm to 1100 μm (Figure 2A). The distal end of the stalk narrows to four cells that provide an anchor to a glandular disc composed of 12 to 16 secretory glandular cells. These disc cells share a subcuticular (apoplastic) cavity that functions as a receptacle for metabolic products from the terpene, flavonoid, and cannabinoid biosynthetic pathways [12,29]. The resulting globular head typically measures ~40 μm to 150 μm in diameter (Figure 2B). During maturation, CSGT morphology undergoes marked changes mostly related to stalk elongation, disc cell growth and division and expansion of the subcuticular cavity [30].
Figure 2.
Structure of a capitate-stalked glandular trichome. Microscope photograph of capitate-stalked glandular trichome (A). Schematic representation of capitate-stalked glandular trichome showing epidermal and hypodermal cells that contribute to the formation of the trichome stalk (B). Specialized stipe cells support the connection between the stalk and the glandular head. Disk-shaped secretory glandular cells and the apoplast cavity are enclosed by a common cuticle. Created in https://BioRender.com.
During the early stages of trichome development in Arabidopsis thaliana, cells undergo cell expansion, endoreduplication, mitotic divisions and coordinated outgrowth, allowing the formation of stalk primordia [21,31]. Evidence suggests that a different mechanism takes place in Cannabis trichome cells. Figure 3 shows how subsequent elongation of the stalk is followed by glandular head enlargement. Finally, around the fifth week after its morphogenesis initiation, glandular trichomes reach the maturity stage, defined by peak cannabinoid accumulation. After maturity, resin secretion through the cuticle takes place, and some capitate-stalked glandular trichomes show glandular head dehiscence, a process that becomes more frequent towards the end of the flowering period [12].
Figure 3.
Capitate-stalked glandular trichome morphogenesis. Cannabis CSGT growth progression is mainly characterized by stalk elongation and glandular head filling with specialized metabolites. Cell fate establishment stage resembles epidermal protuberances that eventually develop a bright cuticle by glandular trichome initiation stage. As CSGT advances to maturity stage, glandular head changes its color from translucid to white and then to yellowish/brown by the time it reaches senescence stage. Created in https://BioRender.com.
Development of CSGT proceeds through four main stages: (i) a sessile stage, (ii) a stalk elongation stage, (iii) a mature stage associated with maximal cannabinoid accumulation, and (iv) a senescence stage that may, but does not necessarily, include dehiscence (rupture) of the glandular head [29,32,33]. Traditionally, CSGT appearance has been used as a floral maturity stage indicator. As illustrated in Figure 3, at early stages, trichomes glandular heads are typically translucent to slightly whitish; then, they shift toward yellow–orange; and by week 8 after flowering transition, they are predominantly dark ochre [34]. The cannabinoid accumulation peak occurs during the early to mid-stages of CSGT maturity, followed by a decline later in development [29,34].
In addition, blue autofluorescence signatures caused by incident light at 430 nm have been correlated with high monoterpene accumulation in capitate-stalked glandular trichomes, while sessile glandular trichomes show red autofluorescence and elevated sesquiterpene content [12,29,33,34].
CSGTs are mainly arranged on the adaxial side of the perigonal bracts of female flowers, the adaxial and abaxial faces of the inflorescence leaves, and, to a much lesser extent, on the epidermis of vegetative leaves and stems [12]. Glandular trichome density increases from the first week of flowering, especially in flower bracts; increments in inflorescence and vegetative leaves have been observed (Figure 4). CSGTs differentiate from sessile trichomes around 15–20 days after flowering onset [35]. Quantitative comparisons among Cannabis genotypes indicate that CSGT densities can range from 20 trichomes/mm2 to 70 trichomes/mm2 [12,33,35] and appear to be associated with genotype, since non-psychoactive hemp-type plants have smaller and fewer stalked glandular trichomes than psychoactive plants [33,35,36].
Figure 4.
Capitate-stalked glandular trichome distribution. Cannabis female bract front view (A). Female bract bearing an immature achene; back view (B). Mature reproductive leaf edge (C). Mature inflorescence leaf adaxial (D) and abaxial plane (E). Immature reproductive leaf nerve detail (F). Immature solitary flower under long-day photoperiod (G). Female flower at four (H) and eight weeks (I) under short-day photoperiod.
These anatomical and developmental features demonstrate that CSGT can be used as indicators of cannabinoid production and floral developmental stage and provide a foundation for nondestructive evaluation of harvest timing and chemical maturity. Recently, deep learning-based image analysis has enabled automated, high-throughput phenotyping of glandular trichomes. Mask R-CNN models can accurately quantify CSGT density from high-resolution micrographs, while complementary workflows segment gland heads in macro/UV images to track maturation-associated fluorescence shifts linked to terpene and cannabinoid dynamics [33,35].
3. Genes Related to Trichome Development in Model Plants
The study of the molecular mechanisms that control the development of glandular trichomes and the biosynthesis of specialized metabolites in model plants has allowed the identification of several genes involved in these processes. Although the specialized literature reflects a wide academic production related to the genetic control of the development of different types of trichomes, recent publications related to capitate glandular trichomes are scarcer, even more so for the species Cannabis sativa L.
3.1. Initiation and Cell Identity Determination
In Arabidopsis thaliana, early stages of trichome morphogenesis are driven by hormonal signaling mainly from the gibberellin, ethylene and jasmonate pathways. Genes encoding C2H2 transcription factors, like ZINC FINGER PROTEIN 6 (ZFP6), ZFP8, GLABROUS INFLORESCENCE STEMS (GIS), GIS2 and GIS3 act upstream of negative trichome regulators like SQUAMOSA PROMOTER BINDING LIKE (SPL9/15), promoting trichome development by integration of gibberellic acid (GA), cytokinin (CK) and ethylene signaling [37,38,39].
Downstream, GLABRA 1 (GL1) (MYB), GL3 (bHLH), and TTG1 (WD40) proteins form a trimeric complex that defines trichome cell identity. This complex activates GL2, whose encoded HD-ZIP protein, GL2, maintains trichome fate and spatial distribution [18,19,20,21]. GL3 is negatively regulated by the E3 ligase UPL3 through the ubiquitin/26S proteasome [40].
LOST MERISTEMS 1/2/3 (LOM) promote trichome formation by modulating SPL activity through protein–protein interactions. LOM1/2/3 transcripts are targeted by miR171 as a mechanism of trichome repression. Complementarily, SPL genes are targeted by miR156, which further promotes trichome formation [41,42]. The double mutant mir172a/b showed early trichome development, suggesting a trichome timing function of miR172 [43]. The TEOSINTE BRANCHED 1, CYCLOIDEA, PROLIFERATING CELL FACTORS (TCP) are trichome branching regulators and promote GIS activation to inhibit trichome cell differentiation. Furthermore, TCP transcripts are targeted by miR319, which likely acts as a trichome positive regulator [44]. Interactions and hierarchy of transcription factors required for Arabidopsis trichome initiation are depicted in Figure 5.
Figure 5.
Comparative regulatory models of trichome development in Arabidopsis thaliana (A), Solanum lycopersicum (B) and Artemisia annua (C). The diagram summarizes major transcriptional and hormonal modules involved in trichome initiation, patterning, growth and glandular differentiation. Color-coded boxes indicate transcription factor families or regulatory categories. Arrows represent positive regulation, red blunt lines indicate repression, and dashed boxes highlight associated gene modules. The comparison shows the transition from the canonical MBW-centered non-glandular trichome model in Arabidopsis toward more modular glandular trichome networks in tomato and Artemisia, where HD-ZIP IV, MYB/MIXTA, bHLH/MYC, WRKY, AP2/ERF and hormone-responsive pathways are increasingly linked to secretory cell differentiation and specialized metabolism.
Hormonal signaling contributes to the early regulation of tomato trichome initiation. More precisely, jasmonate signaling intersects with the core trichome identity network through SlJAZ2, a jasmonate-responsive repressor. Overexpression of SlJAZ2 suppresses jasmonate-mediated trichome development by interfering with the Wo-SlMYC1 module, while additional evidence indicates that jasmonate signaling also affects SlWo and SlCycB2-dependent type I trichome formation [45,46].
Downstream tomato trichome initiation is controlled by a hierarchical regulatory network involving chromatin-associated factors, transcription factors, and cell-cycle regulators. As shown in Figure 5, HAIRPLUS (HAP) functions as an early epigenetic regulator of glandular trichome initiation and cellular identity maintenance. HAP likely functions by modifying chromatin accessibility to favor downstream activation of trichome regulators such as SlWo, SlCycB2, and SlMYC1 [47].
Following this early chromatin-associated step, SlWo acts as a central regulator of multicellular trichome identity. SlWo interacts with the C2H2 zinc-finger protein HAIR (SlH) to promote type I glandular trichome formation, while SlH also interacts with SlZFP8-like and activates SlZFP6, contributing to trichome initiation and identity maintenance [48,49]. The B-type cyclin SlCycB2 is also part of this core developmental module: it acts as a dosage-sensitive cell-cycle regulator and links trichome cell fate with the cell-division program required for multicellular trichome formation [50,51].
In parallel, trichome initiation is further modulated by bHLH and MYB regulators. SlMYC1 functions as a positive regulator of type VI glandular trichome development and regulates terpene biosynthesis in glandular cells [52]. The type VI glandular trichome initiation program is additionally controlled by the SlGRAS9–SlMYC1 module, in which SlGRAS9 directly represses SlMYC1 [53]. More recently, antagonistic MYB regulators have been proposed to fine-tune trichome initiation: SlMYB72 promotes trichome initiation by repressing SlCycB2, whereas SlMYB75 inhibits initiation by activating SlCycB2, with both factors acting through the MYB–bHLH–WD40 regulatory complex [54].
In Artemisia annua, trichome initiation is regulated by HD-ZIP IV and R2R3-MYB factors. Jasmonate induces trichome formation by mediating the ubiquitination and degradation of AaJAZ, leading to the subsequent release of AaHD1. Furthermore, AaHD8 interacts with AaMIXTA1 to positively regulate AaHD1 expression, which is likely necessary for downstream activation of trichome-related genes. Additional evidence supports the positive trichome regulation by AaMIXTA1, as overexpression or silencing of this gene leads to an increase or reduction in trichome density, respectively. AaMYB1 overexpression in A. annua and Arabidopsis leads to increased trichome density; furthermore, silencing of the Arabidopsis homolog, AtMYB66, leads to trichome density reduction in the model plant [55,56,57,58].
Further hormonal control has been addressed by characterization of artemisinin accumulation and trichome density following application of 6-benzylaminopurine (BAP), gibberellic acid (GA3) and jasmonic acid (JA). As expected, JA increased both trichome density and artemisinin content. In contrast, BAP and GA3 showed differential effects on trichome development. BAP strongly increased the density of both filamentous and glandular trichomes, whereas GA3 had a stronger effect on filamentous trichomes. However, both BAP and GA3 had a weaker effect on artemisinin accumulation than JA [59]. In parallel, an additional jasmonate-responsive HD-ZIP IV layer was identified in this pathway: AaPDF2, which is predominantly expressed in glandular secretory trichomes, acts downstream of AaHD1, promotes trichome initiation/density, activates AaGSW2, and antagonizes the negative regulator AaMYB5. Accordingly, AaPDF2 overexpression increases glandular trichome density and artemisinin accumulation, whereas RNAi silencing has the opposite effect [60].
Transcription factors like AaTLR3, AaTAR1, AaMIXTA and AaWIN1, which are linked to lineage commitment, show the highest expression in immature glandular trichome cells (IGC) and stalk cells, while artemisinin pathway transcripts are largely absent [61]. Recently, single-nucleus sequencing revealed that IGCs launch the trichome development program with a housekeeping transcriptome before specialized functions engage [61]. Furthermore, AaWIN1 overexpression leads to increased trichome density, artemisinin biosynthesis and upregulation of AaGSW2 and AaMIXTA1. Additional evidence shows that AaWIN1 interacts with AaMIXTA1, most likely to activate the expression of AaGSW2 [62].
AaTAR1 interacts with cyclins like AaCycTL to control trichome development in Artemisia annua, while, in parallel, promoting cuticle biosynthesis. Overexpression of AaCycTL suppresses trichome density through negative regulation of AaMIXTA1. The co-regulation of AaCycTL/AaTAR1 favors cuticular (non-glandular) trichome formation at the expense of glandular trichome initiation [63]. The regulatory mechanism constituted by AaCycTL, AaTAR1, AaMIXTA1 and AaWIN1 within the trichome initiation stage is depicted in Figure 5.
AaGSW2 is positively regulated by AaHD1/8, and its overexpression results in increased trichome density, whereas Aagsw2 mutants show reduced trichome number and defects in trichome initiation [64,65]. Furthermore, Artemisia annua SQUAMOSA PROMOTER BINDING PROTEIN-LIKE (AaSPL9) positively regulates trichome density and differentiation. Yeast-two-hybrid and luciferase assay studies showed that AaSPL9 promotes trichome development by coupling to the GTAC box of the AaHD1 promoter [66].
Recent work on A. annua seems to retrieve canonical elements of the MYB-BASIC HELIX LOOP HELIX-WD40 (MYB) complex but not completely. AaGL3-like has been identified as a homolog of AtGLABRA3; this transcription factor seems to act upstream and to positively regulate AaHD1 and AaGSW2; RNAi silencing of AaGL3-like reduces glandular trichome density, artemisinin accumulation, and AaHD1 and k transcription levels. As expected, a JAZ factor, AaJAZ8, represses AaGL3-like activity [67]. Another Arabidopsis homolog is AaTTG1, which has been proven to restore the glabrous phenotype of the Arabidopsis ttg1 mutants; moreover, AaTTG1 overexpression increases glandular trichome density in Artemisia annua, most likely through interactions with AaSPL9 [68].
In Nicotiana benthamiana, a B-type cyclin (NbCycB2) can bind the leucine-zipper domain of the tobacco WOOLLY homolog to negatively regulate trichome initiation [69]. Moreover, C2H2 zinc-finger proteins such as NbGIS and NbMYB123-like (MYB homologs) have been implicated in controlling tobacco glandular trichome initiation [70]. Hormonal control of trichome formation has also been demonstrated in tobacco through exogenous application of jasmonic acid (5 mM), which induces glandular trichome formation and upregulates Nicotiana tabacum JAZ genes (NtJAZ1, -3, -5, -7, -8, -9, -10, -12, -15) [71].
Floral trichome initiation in Aristolochia fimbriata appears to depend on a reduced regulatory module centered on GL2, MYB106/MIXTA, RAV1, WIN1, and HDG2-like factors, suggesting that multicellular trichome identity in the perianth is specified by a simpler lineage-specific network than the canonical Arabidopsis pathway [72]. In contrast, Nigella damascena uses the canonical MYB–bHLH–WDR–GL2 module to form short trichomes (ST) and long hairs (LH) on petal epidermis. NidaMYB5-1/-2, NidaGL3, NidaTT8, and NidaGL2 specify trichome identity, while NidaMIXTA governs conical cells rather than ST/LH; silencing of these genes results in failed ST/LH formation. Furthermore, early fate specification by MBW–GL2 is subsequently reinforced by cell-cycle remodeling. This process is driven by endocycle regulators like CPR5-2 and RHL2/HYP6/CCS52A1, which ensure appropriate trichome morphologies [73].
Together, these examples highlight the evolutionary plasticity of trichome regulatory networks, which can either retain the canonical MBW–GL2 architecture or rely on lineage-specific combinations of transcriptional and cell cycle regulators.
3.2. Trichome Density and Spatial Patterning
In Arabidopsis, trichome negative regulators such as TRYPTYCHON (TRY), CAPRICE (CPC), and ENHANCER OF TRYPTYCHON AND CAPRICE (ETC1/2) (R3-MYB type) are synthesized within trichome cells and then exported to adjacent cells to repress trichome initiation and thereby establish proper spacing (Figure 5) [23,74,75]. Subsequently, GL2 maintains the cellular identity of the trichome and its proper spatial patterning [21]. Later GL2 expression is sustained by MYB23 during trichome development. Consistently, gl2-5 mutants display abnormal trichomes, while gl2-5 myb23-3 double mutants fail to form trichomes entirely [76]. Arabidopsis bHLH transcription factors are also important downstream regulators of trichome patterning, as allelic heterogeneity of core bHLH regulators like MYC1 and EGL3 has been shown to alter epidermal pattern and final morphology [77,78,79].
Hormonal regulation plays a crucial role in stabilizing trichome development, integrating jasmonate, auxin and cell-cycle-related pathways during trichome density regulation and differentiation [80]. In this context, auxin signaling appears particularly relevant for trichome abundance, since down-regulation of the auxin response factor SlARF3 reduces the density of type I, V, and VI trichomes, showing that auxin-responsive transcriptional regulation is required to maintain normal trichome patterning in tomato [81]. Jasmonate and auxin signaling in the tomato model are illustrated in Figure 5.
Additional transcriptional modules regulate glandular trichome abundance in a type-specific manner. The SlGRAS9–SlMYC1 module controls type VI glandular trichome formation, with SlGRAS9 acting as a direct transcriptional repressor of SlMYC1. Accordingly, SlGRAS9 knockout or SlMYC1 overexpression increases type VI glandular trichome density and enhances terpenoid accumulation in several tissues [53].
MIXTA and MIXTA-like transcription factors also contribute to epidermal patterning, although their effects appear to be tissue- and paralog-specific. In tomato leaves, SlMIXTA-like has been reported as a negative regulator of leaf trichome development [82], whereas in fruit epidermis SlMIXTA-like activity has been associated with enhanced trichome formation and altered metabolism [83,84]. Mutations in the CUTIN DEFICIENT 2 (SlCD2), an HD-ZIP IV gene, reduce trichome density, suggesting that epidermal differentiation and cuticle-related pathways also contribute to the regulation of tomato trichome patterning [85].
Recently, experiments performed in Artemisia annua identified AaMYC3 as a jasmonate-responsive regulator that increases glandular trichome density by directly activating AaHD1, while also enhancing artemisinin biosynthesis through direct activation of AaCYP71AV1 and AaALDH1 and through interaction with AabHLH1 and AabHLH113 to boost AaADS and AaDBR2 expression, respectively, thereby linking trichome density with metabolic productivity [86]. AaMYB17, AaMYB1, AaMYB16, and AaTAR2 positively regulate trichome development and density, while AaMYB5 acts as a repressor by competing for binding sites on the AaHD1 promoter (Figure 5). TRICHOMELESS REGULATOR 1/2 (TLR1/2) are negative regulators whose overexpression reduces trichome formation by interfering with gibberellic acid signaling [87,88,89].
Other integrators of environmental and hormonal signaling are AaMYB108-like and AaSEPALLATA 1; these genes are differentially expressed following methyl jasmonate applications and light treatments. Furthermore, glucuronidase assay and subcellular localization proved the nature of AaMYB108-like and AaSEPALLATA 1 as trichome-related transcription factors. Gene overexpression and silencing, respectively, showed augmented and diminished glandular secretory trichome density; yet, gene silencing lines still showed trichomes; therefore, it is plausible to think of AaMYB108-like and AaSEPALLATA1 as trichome density regulators [90,91].
Additional A. annua genes such as AaMYC2-type contribute to the regulation of trichome density and artemisinin biosynthesis, most likely by binding to the promoter regions of AaCYP71AV1 and AaADS to activate their transcription; moreover, overexpression and knockdown lines showed that glandular trichome density and artemisinin accumulation correlate with AaMYC2-type expression patterns [92]. Recently, two ABC transporters, AaABCG12 and AaABCG20, were characterized as plasma membrane-localized proteins; moreover, down regulation/overexpression of AaABCG20 resulted in diminished/augmented trichome density, which is likely related to cutin and wax transport during trichome growth. Interestingly, AaABCG2 expression correlates with the overexpression or silencing of upstream transcription factors AaHD1/AaHD8/AaMIXTA1, suggesting that promoter regions of ABC transporter genes can be targeted by these transcription factors [93].
In Aristolochia ringens, trichome distribution is associated with regional specialization of the perianth, with distinct multicellular trichome types developing in the limb, tube, and utricle, consistent with spatially restricted epidermal programs involving genes linked to cell wall formation, wax deposition, and cell proliferation [94]. Spatial trichome patterning across the limb, tube, and utricle is associated with region-specific expression of CINCINNATA TCP genes in the limb and Arin-miR319a/ArinCIN1 in the utricle, together with differential activation of epidermis-related genes such as ArinGRP-like, indicating that distinct perianth domains deploy specialized transcriptional programs to generate different multicellular trichome types [95].
In Camellia sinensis (tea plant), transcriptomic and phylogenetic analysis identified the expression of CsibHLH024 and CsibHLH133 correlated with trichome distribution and co-expressed with CsiTTG1, suggesting their regulatory roles in epidermal development [96]. In Nicotiana tabacum, NtMYB306c acts as a negative regulator of glandular trichome density, as its overexpression suppresses trichome formation and alters the expression of NtJAZ3, NtCycB2, NtHD9, and NtLOX1, linking this R2R3-MYB factor to jasmonate-mediated control of trichome abundance [97]. In Mentha canadensis, heterologous expression of McTTG2 in the Arabidopsis thaliana ttg2-7 mutant increased trichome number and transcriptionally activated AtGL2, AtTRY, and AtBRK1, suggesting that this WRKY factor positively regulates trichome patterning and morphogenesis downstream of the TTG2 module [98].
3.3. Trichome Growth and Morphogenesis
After trichome cell identity is specified, other transcription factors are responsible for regulating the endoreduplication process that supports trichome growth. In Arabidopsis thaliana, the SIAMESE (SIM) gene is an inhibitor of the cyclins (CYCB1;2), which are required to drive complete cell cycles; thus, SIM promotes entry into the endoreduplication cycle [99]. Additional promoters of endoreduplication have been described: constitutive pathogen response 5 (cpr5) mutants exhibit trichomes with higher ploidy levels than the wild-type genotype, and components of the DNA topoisomerase VI complex, including root hairless2 (rhl2) and hypocotyl6 (hyp6), aid progression through the endoreduplication cycle in A. thaliana. Loss-of-function alleles of gl3, kaktus (kak) and try generate trichomes with higher ploidy levels [100]. Overexpression of INHIBITOR/INTERACTOR OF CYCLIN-DEPENDENT KINASES/KIP-RELATED PROTEINS (ICK/KRP) results in low ploidy levels and lethal genotypes [101].
Arabidopsis thaliana TTG2 maintains trichome fate and spacing by directly activating TRY and promotes later morphogenesis through regulation of BRK1, thereby linking patterning with cytoskeletal organization [102]. In parallel, GL3 promotes trichome branching by directly repressing MDP25, a microtubule-destabilizing factor. As illustrated in Figure 5, GL3 acts upstream of FURCA (FRC) genes, showing epistatic interactions with FRC2/4 and additive effects with FRC1/3, showing that branch formation depends on transcriptional control of microtubule stability downstream of the core MBW network [103,104].
Other positive trichome branching regulators such as ANGUSTIFOLIA (AN) and ZWICHEL (ZWI) are responsible for correct microtubule formation and molecular transport by Kinesin microtubule motor proteins; an mutants show that microtubule density is impaired, while the zwi phenotype is characterized by reduced branch number, a contrasting branch phenotype [105,106]. More recently, STICHEL (STI), an AAA-type ATPase/Replication factor C family member, has been proposed as a positive regulator of trichome branch number rather than branch formation; according to evidence, the severity of mutation can produce intermediate phenotypes, and overexpression resulted in hyperbranching [107].
Branching repression in Arabidopsis thaliana is controlled by HD-ZIP IV factors like HDG11/12 since loss-of-function mutants for those genes show a hyperbranching phenotype [108]. Additionally, HDG11 has shown redundant functions with GL2, since transgenic expression of HDG11 driven by the GL2 promoter in a gl2 background partially restores normal branching and trichome induction [76]. R2R3-MYB transcription factors like MYB23 and MYB5 show additive effects, as knockout double mutants result in decreased trichome density on rosette leaves and trichome-impaired branching. Overexpression of MYB5 reduces branching and trichome size, which suggests a complex regulatory network for trichome morphogenesis [109].
Similar to early steps in trichome initiation, tomato glandular trichome growth is driven by an HD-ZIP IV–centered module in which SlWo partners with the cyclin SlCYCB2 and C2H2 zinc-finger factors like HAIR (H/H2/H3/H4) and SPARSE HAIR (SH) to drive repeated cell divisions and stalk elongation [48,50,51,110]. Silencing any of these factors causes a strong reduction or loss of type I glandular trichomes, and the remaining trichomes display shorter stalks, indicating that this module is essential both for initiating and for extending the multicellular stalked glandular trichome program. The phenotypes of sh and h mutants can be restored by the overexpression of ZFP5, suggesting the downstream function of this zinc finger protein [111]. Conversely, overexpression of HAIR-family genes increases both trichome number and stalk length, showing that these zinc-finger proteins act as active positive regulators rather than passive structural components [49].
Cytoskeletal organization is required to confer the characteristic tall, stalked tomato trichome morphology. The HD-ZIP IV transcription factor SlHDZIPIV8 activates HAIRLESS-2, a Nck-associated protein 1-like component of the SCAR/WAVE complex, which promotes actin remodeling. Disruption of either SlHDZIPIV8 or HAIRLESS-2 results in severe deformation and shortening of type I glandular trichomes, linking HD-ZIP IV–mediated control of cytoskeletal dynamics and cell wall assembly directly to proper stalk shape and mechanical stability [112].
Terminal cell differentiation of the secretory head in type VI trichomes requires an HD-ZIP I TF and the SlWo/SlMYC1 complex to regulate cell division and terpene metabolism. In the glandless mutant, loss of function of SlHDZ38 impairs the four-celled glandular formation, leading to reduced volatile terpene accumulation and altered trichome-type composition [113]. In parallel, SlWo/SlMYC1 act as a jasmonate-mediated regulatory mechanism of terpene-biosynthesis genes; additionally, SlMYC1 is presumably related to cell division of the stalk and glandular head of tomato type VI trichomes since knockout lines for this transcription factor result in aberrant trichome structure. In the absence of jasmonate, the SlWo/SlMYC1 complex is likely repressed by SlJAZ2 [45].
As Artemisia annua cells proceed through stalk (SC), basal (BC), and early secretory (SA) identities, the genetic control program shifts toward membrane and cuticle biogenesis: fatty acid, long-chain fatty acid, and wax biosynthetic pathways are activated alongside photosynthetic modules, reflecting high anabolic demand during trichome outgrowth [61]. Late stages of trichome morphogenesis in A. annua are regulated in part by the TRICHOME AND ARTEMISINININ REGULATOR 1 (AaTAR1) gene. RNAi experiments have shown that negative regulation of AaTAR1 results in abnormal glandular trichome morphology [114].
Transcriptome analysis of A. annua seedlings treated with methyl jasmonate and light/dark exposure revealed that genes related to artemisinin biosynthesis are sensitive to this kind of stimulus. Specifically, genes like AaADS, AaCYP71AV1, AaDBR2, and AaALDH1 were upregulated by light and methyl jasmonate treatments, while dark conditions for 24 h decreased their expression levels [115].
Late secretory cell clusters upregulate specialized-metabolism genes. Spatially resolved expression confines artemisinin biosynthesis regulators like AabHLH1, AaMYC2, AaWRKY9, AaBBX21, AaGSW1 and AaWRKY17 to apical/subapical secretory cells, while basal cells (BC) co-express developmental and metabolic regulators like AaHD8, AaABI5, AaERF1 and AaMYB108 [61]. Previous evidence showed that AaWRKY1 co-expresses with AMORPHA-4,11-DIENE SYNTHASE (ADS), which encodes an essential enzyme for artemisinin biosynthesis. In addition, AaWRKY1 binds to the W-box elements of the ADS promoter as observed in Y1H assays, and its overexpression leads to upregulation of most artemisinin pathway-related genes [116].
In Gossypium hirsutum (cotton), transcriptome comparisons of isogenic lines differing in gland development identified COTTON GLAND FORMATION 3 (CGF3) as a key regulator of gossypol-containing glands [117]. More recently, MYB transcription factors were identified in contrasting cotton lines, and virus-induced gene silencing (VIGS) experiments showed that GhMYB4 promotes both gossypol accumulation and gland formation [118]. Conserved motifs in R2R3-MYB proteins were also identified across A. thaliana, A. annua, Solanum lycopersicum, Camellia sinensis and G. hirsutum by multiple sequence alignment. These motifs were used to identify four R2R3-MYB factors in Lavandula spp. with potential roles in trichome development [119].
Comparative transcriptomic analyses in Aristolochia linked multicellular trichome outgrowth to early enrichment of specific cell-cycle regulators—such as AfimCYCA2-4, AfimCDKG-2, AfimE2FA, and AfimASF1A—together with cytoskeleton-related genes including AfimKIN13-A, AfimKIN12-F, AfimPOK2, AfimTUBA1, and AfimARPC5A, suggesting that trichome morphogenesis in this lineage depends on sustained proliferative activity coupled to microtubule and actin-based remodeling rather than on a purely Arabidopsis-like endoreduplication program [94].
Comparative transcriptomics of Cucumis sativus (cucumber) lines RIL-46W and the spontaneous glabrous mutant RIL-46M (csgl3) revealed 711 differentially expressed genes. qPCR validation confirmed roles for CsGL3, CsWIP6, CsTBH, CsHOX3, and CsMYB60 in trichome development. Virus-induced gene silencing (VIGS) experiments demonstrated that CsGL3 regulates trichome density, while CsTBH and CsHOX3 influence trichome morphology [120]. Further studies in cucumber using VIGS validation showed that CsMYC4, -5, -6, -7, and -8 positively regulate glandular trichome density, whereas CsMYC2 acts as a negative regulator [121].
In Salsola ferganica, trichome morphogenesis is shaped by the combined action of phytohormones and cytoskeletal components, with gibberellins strongly affecting trichome length and heterologous expression of SfF-ACTIN and Sfα-TUBULIN altering branching patterns, supporting a major role for cytoskeletal dynamics in trichome growth [122].
4. Transcription Factors Related to Glandular Trichome Development in Cannabis
The regulatory landscape of glandular trichomes in Cannabis is still much less resolved than in Arabidopsis, tomato, or Artemisia, but several recent studies have begun to define its main components. The availability of the Cs10 Cannabis genome has enabled the identification of several members of the MYB and bHLH families, providing a systematic inventory of these transcription factor classes in Cannabis and proposing candidate regulators of cannabinoid pathways based on phylogenetic assignment and expression evidence [123].
Studies of the THCAS promoter sequence showed a 548 bp fragment that drives trichome-specific expression and interaction with transcription factors highly expressed in trichomes like CsAP2L1, CsMYB1, and CsWRKY1. Importantly, CsAP2L1 acted as a positive regulator of THCAS, whereas CsMYB1 and CsWRKY1 behaved as negative regulators, suggesting a model in which cannabinoid biosynthesis is controlled by a regulatory module in coordination with the ongoing CSGT growth [124].
Transcriptomic studies of Cannabis flowers have identified multiple members of the HD-ZIP IV family. Four genes were found to be preferentially expressed in floral tissues: CsHDG5-like, CsGLABRA 2, CsHDG5, and CsANTHOCYANINLESS2. CsGL2 showed differential expression in floral tissues up to 30-fold higher than the other transcription factors. Genes responsible for the fine-tuning of trichome morphogenesis, such as HDG11, HDG2 and PROTODERMAL FACTOR 2, displayed low expression in floral tissues. Furthermore, CsHDG5 transcripts peak around the third week after induction of flowering, which supports the hypothesis that CsHDG5 is involved in trichome development during early floral maturation [125].
Subsequent work identified the CsMIXTA gene as the first transcription factor explicitly proposed to influence Cannabis capitate-stalked glandular trichome density. CsMIXTA is preferentially expressed in Cannabis floral tissues, and its differential expression pattern correlates with flower development and trichome appearance [126]. CsMIXTA shows similarity to AtMYB16 and AaMIXTA; as previously mentioned, these types of transcription factors have fundamental functions within trichome formation and growth, mainly those related to cuticle formation. A strong correlation was also found between CsMIXTA expression patterns and genes related to early stages in the cannabinoid biosynthesis pathway, such as OAC and GPPS [29,125].
Heterologous overexpression of CsMIXTA in Nicotiana tabacum supports a causal effect of this gene on tobacco stalked glandular trichome development, as its overexpression increases trichome density, size, and branching [126]. In contrast, overexpression of CsMIXTA in Arabidopsis thaliana resulted in no significant changes in trichome density or morphology [127]. These contrasting phenotypes suggest that the activity of CsMIXTA is dependent on the regulatory context of the heterologous host. The multicellular glandular trichome network of tobacco may provide regulatory partners or downstream targets that differ from those operating in the unicellular non-glandular trichome pathway of Arabidopsis. Nevertheless, the specific function of CsMIXTA in Cannabis remains to be validated.
Overall, Cannabis appears to control glandular trichome development through MIXTA-like MYB, HD-ZIP IV, SPL, and MYB17 gene modules rather than a single GL1-like master regulator, indicating a species-specific transcriptional program for CSGT density and morphology. These modules identify key hub transcription factors, including a MIXTA-like R2R3-MYB (CsMIXTA-like1), an HD-ZIP IV factor (CsPDF2-like), SPL9, and MYB17, which are proposed to drive initiation and maturation of glandular trichomes. Notably, CsETC1 kept its functions as a strong negative regulator of trichome initiation, whereas CsMYB306 alters trichome architecture by producing hyperbranched, structurally complex trichomes without increasing trichome number [127].
Phylogenetic analysis further supported this model by revealing an expansion of subgroup 9 MIXTA-like R2R3-MYBs in Cannabis together with the lack of a clear GL1-type ortholog. In addition, heterologous assays showed that CsMIXTA did not alter Arabidopsis trichome development, in contrast to its reported effects in tobacco, suggesting partial functional divergence from the canonical Arabidopsis pathway. Consistently, time-course network analysis placed CsML1 and CsPDF2-like within the module most strongly associated with stalked glandular trichome density, supporting their potential participation in early CSGT morphogenesis [127].
More broadly, transcriptome profiling across 8 weeks of female flower development identified 647 transcription factors from 49 families, with ERF, MYB, bHLH, C2H2, WRKY, NAC, GRAS, and bZIP among the most dynamic groups during floral maturation. A co-expression module positively associated with stalked glandular trichome density and cannabinoid accumulation was enriched for genes involved in plant hormone signaling and MAPK signaling, supporting a transcriptionally coordinated developmental program [35]. Gene expression dynamics observed at weeks 2, 4, and 8 indicate key regulatory transitions during floral maturation. Importantly, CsMYC4 expression was found to be strongly correlated with the cannabinoid profile of the plant, the high density of stalked glandular trichomes, the presence of exogenous jasmonic acid, and the increased production of these trichomes in a transgenic tomato line [35].
An additional layer of epigenomic control has recently been associated with glandular trichome regulation in Cannabis. Active histone marks such as H3K4me3 and H3K56ac are enriched in trichomes and correlated with trichome-specific gene expression, whereas H3K27me3 and H2A.Z are linked to repression in non-trichome tissues. Trichome-specific cis-regulatory elements have been associated with genes involved in cannabinoid and terpene biosynthesis, metabolite transport, and trichome maturation, suggesting that glandular trichome identity depends not only on transcription factors, but also on a specific chromatin structure that enables tissue-specific transcriptional programs [128].
Recently, ethephon-induced feminization of genetically male (XY) Cannabis flowers was shown to activate a glandular trichome program that is normally absent from untreated male inflorescences, and this correlates with up-regulation of the trichome initiation regulators ZFP5 and GL1 and repression of the negative regulator TPL. In this system, most other canonical trichome regulators (e.g., GL2, GL3, TTG1) are not upregulated at early floral stages, indicating that ethylene is sufficient to turn on the upstream “initiation switch” but not the full maturation cascade: induced female flowers accumulate cannabinoid-rich glandular trichomes that are predominantly sessile with ~8 disc cells and enriched in CBCA/β-caryophyllene, rather than the highly productive capitate-stalked trichomes with >8 disc cells typical of mature XX female flowers [13].
Recent transcriptomic analysis of CSGT stalk and glandular head showed a differentially specialized transcriptome with 6018 genes and 35 proteins strongly expressed in the trichome stalks. Enriched categories in the stalk transcriptome include exporters, importers, companion cells, bundle sheath, xylem and procambium. Analysis show that trichome stalks are characterized by a growth and vascular-related transcriptomic signature [129].
New evidence shows that CsYABBY3 affects specialized metabolism and trichome density. Transient overexpression of CsYABBY3 in Cannabis leaves and hairy roots leads to increased CBD and CBG accumulation; this effect is likely the result of CsYABBY3 and ASYMMETRIC LEAVES 1 (CsAS1) dimerization to subsequently bind to the promoters sequences of AROMATIC PRENYLTRANSFERASE 4 (CsPT4) and CsCBDAS to positively regulate them. Furthermore, overexpression of CsYABBY3 in a tomato heterologous system increased both glandular and non-glandular trichome density. When compared to the control lines, glandular trichome proportion was higher in overexpression lines [130]. Evidence coming from comparative analysis of glandular trichome transcriptomic atlases from different species bearing glandular trichomes including Cannabis, revealed conserved trichome regulatory components including TFs like HD-ZIP IV and GL1-like [131].
By integrating the available evidence, a model for the genetic regulation of capitate-stalked glandular trichome development in Cannabis is proposed. The model presented in Figure 6 is organized as a developmental progression from epidermal cell-fate specification to trichome maturation and specialized metabolism. At early stages, candidate regulators from several transcription factor families, including MIXTA-like MYBs, HD-ZIP IV, C2H2 zinc-finger proteins and GL2-related factors, are proposed to participate in trichome initiation and epidermal differentiation, whereas repressors such as CsETC1 may restrict trichome fate in neighboring cells. Jasmonate signaling may further modulate this early regulatory network through CsJAZ-dependent repression of factors such as CsMYC4 and MYB17. A subsequent developmental transition potentially involves CsSPL9-like together with the CsYABBY3–CsAS1 module, followed by regulators associated with glandular trichome architecture, including CsMIXTA, CsMYB306 and CsHDG11. During maturation, transcriptional control becomes increasingly coupled to specialized metabolism, with CsAPL21, CsMYB1, CsMYC4 and CsWRKY1 linked to the regulation of cannabinoid biosynthetic genes.
Figure 6.
Proposed regulatory model of capitate-stalked glandular trichome development in Cannabis. The diagram summarizes candidate regulatory modules involved in each stage of trichome development. Color-coded boxes indicate transcription factor families or regulatory categories. Arrows represent positive regulation, and red blunt lines indicate repression. Solid lines indicate direct evidence in Cannabis, dashed lines indicate functional evidence from heterologous systems, and dotted lines denote proposed or incompletely resolved interactions. Weeks 1–4 represent an approximate developmental progression during early floral maturation. The model highlights a modular regulatory architecture in which MIXTA-like MYB, HD-ZIP IV, bHLH/MYC, YABBY–AS1, AP2/ERF, WRKY and C2H2-ZFP factors may coordinate glandular trichome development with cannabinoid pathway activation.
Rather than representing a single linear pathway, the proposed model depicts partially overlapping regulatory modules controlling trichome initiation, developmental transition, architecture and metabolic maturation. Importantly, several of these relationships remain hypothetical or are supported primarily by expression, interaction or comparative evidence and therefore require direct functional validation in Cannabis.
To facilitate comparison among the proposed regulators discussed above, Table 1 summarizes their putative developmental roles, the type of evidence currently available in Cannabis, and the degree of functional support provided by heterologous or molecular assays. Because the available studies differ in the trichome phenotype examined, we distinguish glandular trichomes in general (GTs), stalked glandular trichomes (SGTs), and capitate-stalked glandular trichomes (CSGTs), according to the terminology and level of morphological resolution reported in each study.
Table 1.
Proposed regulators of Cannabis glandular trichome development and supporting evidence.
5. Genetic Regulation of Specialized Metabolism in Cannabis Glandular Trichomes
Among the specialized metabolites synthesized by CSGTs, there is a wide variety of cannabinoids and terpenes. The most abundant synthesized cannabinoids are THCA, CBDA, CBGA, cannabichromenic acid (CBCA), and cannabinol (CBN), although more than 100 additional cannabinoids have been described in Cannabis [16,29,132,133].
Transcriptomic studies indicate that Cannabis capitate-stalked glandular trichomes (CSGTs) are highly specialized secretory tissues with a distinct expression profile. In the Cannbio atlas, trichomes showed 1479 differentially expressed genes relative to whole female flowers, including enrichment of CBDAS, THCAS, lipoxygenases, and other specialized metabolism genes [134]. During maturation, trichome transcriptomes shift toward stronger activation of cannabinoid- and terpene-related pathways, while multi-cultivar comparisons confirm a conserved trichome signature with coordinated up-regulation of LOX, OAC, APT, THCAS, and CBDAS [134,135].
Proteomic profiling depicts trichome heads as highly active secretory tissues marked by functional specialization toward secondary metabolism, with enrichment of proteins directly associated with cannabinoid and terpenoid production, including CsPT4/CBGAS, CsPT3, chalcone isomerase, and MEP-pathway enzymes such as DXS, DXR, and MCT. Across 1820 proteins identified overall, 1240 were detected in head isolates, compared with 396 in stalks and 1682 in late flowers, reinforcing the biochemical distinctiveness of the head fraction. At the same time, this specialization appeared to be coupled to elevated energetic, transport, and redox demands, consistent with enriched ATPases and head-specific ABC/PDR-type transporters [136].
Metabolome–proteome profiling of isolated CSGT over five weeks (W3–W8) reveals a functional peak at W6, where THCA and central-carbon flux (glycolysis/pyruvate/TCA) peak together with a timed plastid import/MEP program. Distinct enzyme kinetics further shape the molecular landscape: tetraketide synthase (TKS) rises at W6, prenyltransferase 1 (PT1) emerges as a candidate control point, while Olivetolic acid cyclase (OAC) stays relatively stable; THCAS surges at W6 as sesquiterpenes peak earlier (~W5) and monoterpenes shift later (toward 8), indicating partially decoupled terpene modules across development [30].
CSGTs also display transcriptional rewiring of primary metabolism to support high flux toward specialized metabolites. Positive differential expression of GLUCOSE-6-PHOSPHATE ISOMERASE (GPI) and FRUCTOSE-BISPHOSPHATE ALDOLASE (ALDO) has been reported, increasing the availability of glucose and glyceraldehyde-3-phosphate metabolites that can be used in the methylerythritol 4-phosphate (MEP) biosynthetic pathway and as a substrate for NADPH production via glyceraldehyde-3-phosphate dehydrogenase [17,29,137]. Concomitantly, downregulation of phosphoglycerate kinase (PGK) coding genes is observed in trichomes, suggesting a metabolic shift that favors NADPH production over NADH and ATP as cofactors [135,138,139]. This shift is consistent with the high reducing power required for terpene and cannabinoid biosynthesis.
Positive differential expression of genes encoding pyruvate kinase (PK)-type enzymes and negative regulation of the gene encoding phosphoenolpyruvate carboxylase (PEPC) have also been reported; this transcriptional control is associated with increased acetyl coenzyme A (AcCoA) through pyruvate dehydrogenase (PDH) [135]. The upregulation of these genes likely reflects the metabolic demand for cofactors necessary for terpenes and cannabinoids biosynthesis.
Genes such as 1-DEOXY-D-XYLULOSE 6-PHOSPHATE SYNTHASE (CsDXS1), HMG-COA REDUCTASE (CsHMGR2), and farnesyl diphosphate synthase (CsFPPS2) are expressed in the glandular trichomes. Some genes are specific to different stages of inflorescence maturation. For example, genes of the MEP biosynthetic pathway are preferentially expressed at advanced flowering stages, whereas those expressed at early flowering stages are related to the mevalonate pathway (MEV), prenyltransferases, and terpene synthases [134].
Terpene accumulation is also spatiotemporally regulated during the Cannabis life cycle. In chemotypes I, II, and III, sesquiterpenes such as β-caryophyllene and humulene are primarily enriched in leaves, with maximal accumulation around day 60. In contrast, monoterpenes including myrcene and limonene are significantly more abundant in flowers, especially from day 60 to day 90, coinciding with the maturation of glandular trichomes. Chemotype I shows the highest monoterpene concentrations during late flowering, while chemotype III presents a more balanced profile. These patterns indicate a developmentally regulated activation of terpene biosynthesis, likely driven by trichome density and gene expression dynamics [140].
It has been established that monoterpenes accumulate in Cannabis glandular trichomes at higher proportions than sesquiterpenes [29]. Reported monoterpenes include β-pinene, α-pinene, β-tujene, 3-carene, terpinolene, limonene, terpineol, 1,8-cineole, α-terpinene, linalool, myrcene, and (Z)-β-ocimene [141,142]. Among the most abundant sesquiterpenes, the following are representative: α-elemol, (E)-β-farnesol, (E)-β-farnesene, bisabolol, (+)-α-bergamotene, δ-cadinene, γ-eudesmol, valencene, eremophyllene, β-himachalene, α-guaienene, germacrene D, alloaromadendrene, and β-caryophyllene [29,141,142].
At single-trichome resolution, genotype effects are clear: Cannabis (chemotype III) trichomes accumulate far more CBDA (~2.0–5.7 µg per trichome) and higher THCA than chemotype II. Furthermore, chemotype II trichomes uniquely presented Δ8-THC. Despite these absolute shifts, the CBD:THC ratio remained stable between single trichomes and whole inflorescences within each genotype, indicating strong chemotype-level genetic control [143].
6. Experimental Tools for Dissecting Regulatory Networks in Cannabis
The first methodological steps toward dissection of regulatory networks in Cannabis require the development of an experimental toolbox adapted to the species. Several protocols are now available for tissue culture, Agrobacterium sp.-mediated transformation, gene silencing, cellular localization, transient gene expression, protein and gene interactions validation, among others.
A major advance was the establishment of a virus-induced gene silencing (VIGS) platform, which used genome/transcriptome assisted identification of PDS and ChlI, prediction of siRNA targets, agroinfiltration-mediated delivery, and qPCR validation to demonstrate the first transient gene knockdown in Cannabis, with transcript reductions of about 70–73% and visible bleaching phenotypes [144]. In parallel, cell-type-specific network analysis became possible through RNA-seq of 27 trichome libraries, de novo transcriptome assembly, metabolite profiling, co-expression analyses of cannabinoid and terpenoid pathways, cloning and functional characterization of terpene synthase candidates [145].
Soon after, a vacuum agroinfiltration protocol for aerial tissues was reported. The protocol was validated by silencing of the PHYTOENE DESATURASE (PDS) gene, which produced an albino phenotype and reduced transcript levels, including in trichome-bearing organs [146]. Subsequently, cultivar dependence and transformation recalcitrance were further addressed. DMG278 was selected as a highly regenerating line; furthermore, shoot regeneration was boosted through transformation with constructs carrying developmental regulators, including GROWTH REGULATING FACTOR (GRF) and GRF-INTERACTING FACTOR (GIF), and a CRISPR system targeting the PDS gene [147]. These approaches provide transient and stable routes to test candidate genes, including those regulators of glandular trichome development and metabolism.
Eventually, short-cycle transient transformation in Cannabis seedlings further increased throughput for construct screening, making it feasible to pre-test regulators, reporters and effectors before committing to slower workflows. The Agrobacterium strain AGL1 was selected for a vacuum-assisted agroinfiltration protocol for Cannabis seedling transformation because it showed higher transformation efficiency than other tested strains, including GV3101, EHA105 and LBA4404. Interestingly, the RUBY reporter system was proven to be a fast and practical tool for transformation monitoring, showing results within five to seven days after inoculation and with no specialized equipment required to visualize results [148].
Recent advances in protoplast isolation and transformation techniques have enabled a wide range of molecular applications in plants, including transient gene expression, genome editing, subcellular localization, and the study of gene–gene and protein–protein interactions. The first adaptation of this approach to Cannabis was derived from established Arabidopsis thaliana protoplast protocols. This technique proves to be effective for studying transcription factor activity using an auxin-responsive reporter construct, DR5::GFP. Treatment with 5 µM indoleacetic acid (IAA) was reported to produce a ~4-fold increase in GFP fluorescence relative to a constitutive p35S::GFP control, validating protoplasts as a platform for hormone-responsive gene regulation assays in Cannabis [149].
This system was validated by demonstrating nuclear localization and transcriptional activity of CsMYC2, a Cannabis bHLH transcription factor, and confirmed its applicability across eight genetically diverse Cannabis cultivars [96]. Subsequent refinements improved digestion and uptake by incorporating pectolyase and vacuum infiltration [150]; these improved systems were then used not only for reporter-based assays but also for subcellular localization of key cannabinoid-pathway enzymes, including CsCBCAS, CsCBDAS, and CsTHCAS, thereby establishing Cannabis protoplasts as a potential platform for construct testing and gene function analysis [151].
A more recent protocol for hemp protoplast isolation was reported for cultivars Finola and Futura 75; notably, phytosulfokine application and an alginate matrix improved the frequency of protoplast-derived callus. This was further complemented by standardization of protoplast transfection, which showed that a higher concentration of the pX08YPet plasmid proportionally increased the transformation efficiency. So far, Cannabis plant regeneration remains elusive or has a low-success-rate procedure at best; after four weeks, callus showed signs of necrosis, and by eight weeks, none of the tested lines were able to form shoots. Still, protoplast-derived callus remains a robust system to test gene functions and genetic networks related to complex traits [152].
Complementary methodological advances came from combining promoter dissection, heterologous reporter assays, yeast one-hybrid screening, and transient transactivation tests to move from candidate-TF prediction to direct regulatory inference. This approach has enabled the determination of trichome-specific expression of THCAS in trichomes of Arabidopsis, identification of transcription factors via Y1H screening of cDNA libraries, and cellular localization of candidate regulators [124]. Recently, a ratiometric system for the assessment of promoter activity in Cannabis was reported. The method relies on agroinfiltration-based transient gene expression: GUS-TS3337, a thermoresistant variant of glucuronidase driven by the NOS promoter, and a wild-type GUS driven by the promoter to be tested. After heat treatment of control samples, promoter activity is quantified by performing a 4-methylumbelliferone (4-MU) fluorometric assay. Hence, it provides a fast, simple and relatively cheap platform to test promoter activity [153].
Although the knowledge about genetic control of Cannabis trichomes is still being assembled, some Cannabis genes and transcription factor families related to trichome morphogenesis have been identified. Those genes are main candidates for study using protoplast systems assisted by reporter genes, among other systems, to dissect these genetic networks. At the same time, orthologs from model and crop species provide guidance about which regulatory modules (HD-ZIP IV, R2R3-MYB/MIXTA-like, bHLH, JAZ/MYC, SPL, etc.) are most likely to control trichome initiation, identity, and maturation in Cannabis. This comparative framework not only narrows the set of high-priority genes to study experimentally but also supports the construction of working in vitro models for cell identity specification and developmental progression of capitate-stalked glandular trichomes (Figure 6).
7. Cannabis Has Rewired the Genetic Control of Glandular Trichome Development
Despite the advances presented here, our current understanding of trichome biology in Cannabis raises more questions than answers. For example, the factors that limit the development of capitate glandular trichomes in male plants, and in non-floral tissues of female plants, remain unresolved. The ability to manipulate these limiting factors could enable the enhancement of cannabinoid accumulation in tissues that normally do not support high densities of productive trichomes [154].
Taken together, the comparison among Arabidopsis thaliana, Solanum lycopersicum, Artemisia annua and Cannabis indicates that trichome development is controlled by a partially conserved but highly rewired regulatory toolkit. In Arabidopsis, the developmental program is centered on the canonical MYB–bHLH–WD40 complex, followed by downstream regulators such as GL2, TTG2, R3-MYB repressors, endoreduplication factors and cytoskeleton-remodeling genes. This model has been useful for defining the logic of epidermal cell fate specification, but it mainly describes non-glandular trichome development. In contrast, tomato and Artemisia illustrate how the same transcription factor families can be reorganized into glandular trichome networks in which MIXTA-like MYBs, HD-ZIP IV factors, MYC/bHLH proteins, C2H2 zinc fingers, AP2/ERF, WRKY and hormone-responsive regulators acquire stronger roles in secretory cell differentiation and specialized metabolism.
Cannabis appears to follow this second logic rather than the canonical Arabidopsis model. Current evidence does not support a fully resolved Cannabis MYB–bHLH–WD40 complex equivalent to GL1–GL3/EGL3–TTG1. Instead, available studies point to a modular regulatory architecture involving MIXTA-like MYBs, HD-ZIP IV factors, SPL9-like and MYB17 candidates, CsMYC4, CsYABBY3–CsAS1, and AP2/MYB/WRKY regulators of cannabinoid biosynthetic genes. This would suggest that Cannabis glandular trichome development is not controlled by a single GL1-like master regulator, but by partially overlapping modules that regulate initiation, density, morphogenesis, glandular maturation and cannabinoid biosynthesis.
Additional information is necessary to comprehend the genetic control governing how the initial trichome cell chooses a developmental program among the glandular and non-glandular morphologies. In tomato, SlWo, an HD-ZIP TF, plays an important role within a complex system of feedback signaling. As Wooly accumulates, it promotes its own transcriptional activation and that of the MULTICELLULAR TRICHOME REPRESSOR 1 (MTR) gene, which acts as a repressor of SlWo. Downstream, the high SlWo accumulation pathway is characterized by activation of MIXTA1 and SlWox3b, which favors the formation of digitate trichomes; on the contrary, low SlWo accumulation results in activation of the LEAFLESS (LFS) gene and therefore in peltate trichome development [155]. Furthermore, high and low levels of SlWo have also been correlated with trichome stalk-cell division and endoreduplication, respectively [156].
Since HD-ZIP TFs seem to gain relevance within the genetic control programs of trichome morphogenesis within species having glandular and non-glandular trichomes, it is at least plausible to consider that Cannabis presents a Woolly orthologue that perhaps also works in a dosage-dependent manner; such a system could be partially accountable for the different phenotypes of glandular trichomes (sessile and stalked) and for the hair-like trichome as well.
MYB transcription factor family is already known to influence cannabinoid pathway kinetics, yet the precise regulatory relationships between candidate MYB genes and genes required for metabolite accumulation have not been fully defined. MYB transcription factors are widely distributed in other model plants, and their role in trichome development has been described previously; therefore, it is highly probable that several MYB transcription factors modulate Cannabis trichome morphogenesis as well [157]. In a similar way, CsYABBY3 is required for both the cannabinoid pathway and glandular trichome formation [130], suggesting that morphogenesis and onset of specialized metabolism can be parallel processes.
Some regulators related to glandular trichome morphogenesis are also linked with cannabinoid and terpene biosynthesis, suggesting that these processes may be controlled by partially overlapping regulatory networks. It is plausible to consider a hypothetical feedback-based mechanism in which specialized metabolism influences glandular trichome development; however, there is currently no direct evidence in Cannabis supporting such a causal relationship. The increase in cannabinoid accumulation from the first week of flowering, followed by an increase in CSGT density between the second and fourth weeks of floral development [35], is consistent with coordinated regulation of these processes but does not establish their causal direction. Interestingly, this hypothetical coordination resembles the tomato WO/SlMYC1 complex in which both factors positively regulate terpene biosynthesis and SlMYC1 individually promotes cell division and expansion [45]. Other examples of regulatory overlap include trichome morphogenesis-related genes like GhMYB4 and AaTAR1, which are also involved in gossypol and artemisinin accumulation, respectively [114,118].
A central conclusion emerging from the four models is that glandular trichome development and specialized metabolism are deeply interconnected. Therefore, Cannabis trichomes should be understood not only as epidermal structures but as developmentally programmed metabolic organs. Still, high density of CSGT should not be interpreted as a direct indicator of chemotype, since cannabinoid accumulation is, to a certain extent, the result of the allelic combination of the genes involved in the cannabinoid pathway.
As shown by previous work, the carbon chain length of the cannabinoid molecular structure is determined by the polygenic A locus, which has the Ape1-n and Apr1-n alleles. The enzyme they encode preferentially uses butanoate and hexanoate substrates, respectively [158]. The absence of cannabinoids is explained by the action of a locus that segregates independently and affects the synthesis of cannabinoid phenolic precursors. This locus has been described as the O locus, and in the homozygous dominant O/O state, it allows the synthesis of phenolic precursors, while in the recessive o/o state, it does not [159].
Additional complexity is added by considering the sequence heterogeneity of the genes encoding the THCAS and CBDAS enzymes [159]. Previous evidence shows that the distribution of 25 single nucleotide polymorphisms (SNPs) between positions 136 and 869 of the THCAS sequence can affect THCA accumulation. Similarly, CBDAS sequences exhibit at least eight polymorphic loci between positions 407 and 704 that can be correlated with CBDA accumulation [158]. This information has proven to be valuable to the aim of discriminating between drug type and fiber (hemp) type plants, as molecular markers relying on SNP configuration of THCAS and CBDAS have been successfully implemented [160,161,162].
Considering the above, it is likely that chemotype is the result of interaction between parallel genetic control networks and their allelic combinations rather than the contribution of a reduced group of genes. Moreover, the existence of high/moderate trichome-density Cannabis plants with a poor or null cannabinoid accumulation profile can be supported by the presence of SNPs with moderate to high-impact alterations of amino acid chains that modify the secondary and tertiary structure of the THCAS/CBDAS enzymes [161]. Therefore, glandular trichome density and metabolic output should be treated as related but non-equivalent traits. Furthermore, trichome density and cannabinoid accumulation are influenced by sampled organ, floral developmental stage, and environmental or cultivation conditions; as a consequence, the relationships discussed here should be regarded primarily as qualitative trends rather than as universal quantitative associations between trichome density and cannabinoid content.
The comparison among models further indicates that transcription factors alone are insufficient to explain the Cannabis phenotype. Hormonal signaling, especially jasmonate and ethylene, appears to interact with developmental regulators, while recent epigenomic evidence suggests that trichome-specific chromatin states may define which biosynthetic and developmental genes can be activated. This is consistent with tomato HAP-mediated chromatin regulation and with the strong influence of light, jasmonate, gibberellin and cytokinin-related signals in A. annua. Therefore, Cannabis glandular trichome identity likely emerges from the integration of transcription factor modules, hormone signaling, chromatin accessibility and floral developmental context.
The applied relevance of this regulatory network is already evident. Patents involving heterologous expression of A. annua MYB genes in Cannabis demonstrate that trichome density and secondary metabolite modulation are recognized as valuable targets for cannabinoid production. Currently, three patents involving the expression of heterologous systems containing A. annua MYB family genes in Cannabis have been claimed for the purpose of trichome density and secondary metabolite modulation: US20190352662A1, WO2019147873A2, and US10724048 B2 [163,164,165]. This confirms that trichomes are important structures for the yield of cannabinoids per plant and therefore for the industrial production of these metabolites within the medicinal and recreational Cannabis economic sector.
However, these translational applications also emphasize the current knowledge gap: most Cannabis candidate regulators remain supported by transcriptomic association, promoter interaction, heterologous assays or correlative evidence rather than direct functional validation in Cannabis. Moving from candidate genes to causal regulatory models will require Cannabis-specific perturbation approaches, including promoter–reporter assays, hormone treatments, transient expression, stable transformation, CRISPR-based editing, automated phenotyping and cell-specific metabolic assays. In this sense, the comparative models from Arabidopsis, tomato and Artemisia do not provide a finished explanation for Cannabis, but they define a rational framework for testing how conserved transcriptional families have been rewired to generate cannabinoid-rich capitate-stalked glandular trichomes.
Other transcription factors may be responsible for related phenomena such as sex determination and trichome development, including FT (Flowering Locus T), FY (Flowering Time control protein), PIN2 (Auxin efflux carrier component 2), CRL5 (AP2-like ethylene responsive transcription factor), and TBL6 (Protein trichome birefringence-like 6) [132]. Those factors belong to upstream or parallel genetic networks that are well differentiated from the ones controlling glandular trichome formation.
Comparison of the genetic network controlling glandular trichome morphogenesis among different species evidenced a modular and highly specialized machinery that can be depicted as (i) integration of hormonal and environmental signaling, (ii) initiation, (iii) repression of trichome fate in neighboring cells, (iv) growth, (v) cell division, (vi) secretory cell formation and (vii) secondary metabolite biosynthesis. Moreover, independent transcriptome analyses have shown considerable differences among gene expression patterns of glandular trichomes and floral tissues; even between the trichome stalk and the glandular head, the gene expression programs are different, reflecting the specialization of each part of the trichome structure.
Considering that genes controlling trichome morphogenesis belong to a relatively specific and well-defined subset of transcription factors, at least in the most detailed models, it is possible to consider approaches in which trichome morphogenesis is induced without the previous development of any floral tissue or even a whole plant. Implementation of a hypothetical combination of plant growth regulators, inductive photoperiod, light intensity, nutrient supply and trichome-related gene modulation, applied to an undifferentiated cell mass (callus) could result in a vegetal mass rich in trichomes and therefore in a biological metabolite battery. Although untested in Cannabis, trichomes have been reported to develop on Artemisia annua callus, accompanied by stage-dependent expression of trichome-associated genes [166], suggesting that trichome developmental programs can be activated in callus-derived tissue. Such a biological structure offers the possibility not only to produce cannabinoids or terpenes, but also specialized metabolites from different organisms, as long as metabolic pathways can be reconstructed in undifferentiated Cannabis cells, allowing the potential of glandular stalked trichomes to be harnessed as biological micro refineries.
The isolation and short-term culture of disc cells from capitate-stalked glandular trichomes offers an innovative, cell-autonomous assay to probe how signals rewire cannabinoid factories without the confounding effect of changing trichome numbers. Recent work shows that disc cells treated with phytohormones like kinetin, jasmonic acid, salicylic acid, ethylene, and inhibitors like diethyldithiocarbamic acid (DIECA) exhibit large, convergent proteome shifts, related to remodeling plastid import/trafficking, cytosolic acetyl-CoA control, and very-long-chain fatty-acid/cuticle pathways. This disc-cell platform thus enables mechanism-focused screening—separating density effects from metabolic capacity—and nominates organelle transport and carbon partitioning as actionable levers for future engineering [167].
Further refinement, such as the integration of suspension cell cultures, could expand their utility for exploring the impact of genetic engineering on cannabinoid production and other metabolic pathways [168].
Finally, different reports in the literature indicate that Cannabis genetic transformation using Agrobacterium tumefaciens is feasible, and this is emerging as a key enabling technology for both basic and applied studies. Agrobacterium-mediated transformation would also allow the implementation of targeted gene editing using CRISPR–Cas systems [27,169,170]. The transfer of established molecular tools from other species, such as transient expression systems, promoter–reporter assays, hormone-based modulation, and CRISPR-based editing, together with the strong economic incentive provided by legalization and commercialization, is likely to drive rapid progress in dissecting the genetic and developmental control of capitate-stalked glandular trichomes in Cannabis.
Overall, three main conclusions emerge from the comparative evidence reviewed here. First, glandular trichome development in Cannabis appears to rely on a modular and partially rewired regulatory network rather than on a direct equivalent of the canonical Arabidopsis trichome pathway. Second, trichome morphogenesis and specialized metabolism are closely interconnected, although trichome density alone should not be considered a direct predictor of cannabinoid accumulation or chemotype. Finally, most proposed regulatory relationships in Cannabis still require direct functional validation. Comparative models from Arabidopsis, tomato, and Artemisia therefore provide a valuable framework for identifying candidate regulators, but Cannabis-specific genetic, molecular, and physiological approaches will be essential to establish causal mechanisms and ultimately enable the targeted engineering of cannabinoid-producing glandular trichomes.
Author Contributions
Conceptualization, J.D.R.B., F.S. and H.G.; writing—original draft preparation, J.D.R.B.; writing—review and editing, F.S. and H.G.; visualization, J.D.R.B.; supervision, H.G. and F.S.; project administration, H.G.; funding acquisition, H.G. All authors have read and agreed to the published version of the manuscript.
Funding
This work was supported by the Natural Sciences and Engineering Research Council (NSERC) of Canada (RGPIN 2020-00402) and the Université du Québec à Trois-Rivières—H.G. laboratory.
Data Availability Statement
No new data were created or analyzed in this study. Data sharing is not applicable to this article.
Conflicts of Interest
The authors declare no conflicts of interest.
Abbreviations
The following abbreviations are used in this manuscript:
| CRISPR | Clustered Regularly Interspaced Palindromic Repeats |
| Cas | CRISPR-associated protein |
| RNA | Ribonucleic acid |
| DNA | Deoxyribonucleic acid |
| Y1H | Yeast one-hybrid |
| Y2H | Yeast two-hybrid |
| CHIP | Chromatin immunoprecipitation |
| Seq | Sequencing |
References
- APG. An update of the Angiosperm Phylogeny Group classification for the orders and families of flowering plants: APG IV. Bot. J. Linn. Soc. 2016, 181, 1–20. [Google Scholar] [CrossRef] [Scilit]
- McPartland, J.M. Cannabis Systematics at the Levels of Family, Genus, and Species. Cannabis Cannabinoid Res. 2018, 3, 203–212. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- McPartland, J.M.; Hegman, W.; Long, T. Cannabis in Asia: Its center of origin and early cultivation, based on a synthesis of subfossil pollen and archaeobotanical studies. Veg. Hist. Archaeobotany 2019, 28, 691–702. [Google Scholar] [CrossRef] [Scilit]
- Mediavilla, V.; Jonquera, M.; Schmid-Slembrouck, I.; Soldati, A. Decimal code for growth stages of hemp (Cannabis sativa L.). J. Int. Hemp Ass. 1998, 65, 68–74. [Google Scholar]
- Kundan, M.; Gani, U.; Nautiyal, A.K.; Misra, P. Molecular Biology of Glandular Trichomes and Their Functions in Environmental Stresses. In Molecular Approaches in Plant Biology and Environmental Challenges; Springer Nature: Singapore, 2019; pp. 365–393. [Google Scholar]
- Small, E. Evolution and Classification of Cannabis sativa (Marijuana, Hemp) in Relation to Human Utilization. Bot. Rev. 2015, 81, 189–294. [Google Scholar] [CrossRef] [Scilit]
- Passardi, F.; Dobias, J.; Valério, L.; Guimil, S.; Penel, C.; Dunand, C. Morphological and physiological traits of three major Arabidopsis thaliana accessions. J. Plant Physiol. 2007, 164, 980–992. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kaur, S.; Khanal, N.; Dearth, R.; Kariyat, R. Morphological characterization of intraspecific variation for trichome traits in tomato (Solanum lycopersicum). Bot. Stud. 2023, 64, 7. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, Z.; Li, X.; Zhao, Y.; Jin, Y.; Zhou, J.; Huang, L.; Zha, L.; Yuan, Y. Microscopic characterization of five Artemisia crude herbs using light microscopy, scanning electron microscopy, and microscopic quantitative analysis. Microsc. Res. Tech. 2022, 85, 2428–2437. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dayanandan, P.; Kaufman, P.B. Trichomes of Cannabis sativa L. (cannabaceae). Am. J. Bot. 1976, 63, 578–591. [Google Scholar] [CrossRef] [Scilit]
- Raman, V.; Lata, H.; Chandra, S.; Khan, I.A.; ElSohly, M.A. Morpho-Anatomy of Marijuana (Cannabis sativa L.). In Cannabis sativa L.-Botany and Biotechnology; Chandra, S., Lata, H., Elshoy, M., Eds.; Springer International Publishing: Cham, Switzerland, 2017; pp. 123–136. [Google Scholar]
- Punja, Z.K.; Sutton, D.B.; Kim, T. Glandular trichome development, morphology, and maturation are influenced by plant age and genotype in high THC-containing Cannabis (Cannabis sativa L.) inflorescences. J. Cannabis Res. 2023, 5, 12. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Garcia-de Heer, L.; Guo, Q.; Mieog, J.; Nolan, M.; Liu, L.; Dimopoulos, N.; Melzer, R.; Kretzschmar, T. Transcriptomic analysis of ethephon-induced sex reversion of male Cannabis sativa reveals changes in expression of floral homeotic genes and a distinct trichome morphology. J. Exp. Bot. 2025, 76, 5401–5418. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ghosh, D.; Chaudhary, N.; Shanker, K.; Kumar, B. Journal of Applied Research on Medicinal and Aromatic Plants Monoecious Cannabis sativa L. discloses the organ-specific variation in glandular trichomes, cannabinoids content and antioxidant potential. J. Appl. Res. Med. Aromat. Plants 2023, 35, 100476. [Google Scholar]
- Stack, G.M.; Toth, J.A.; Carlson, C.H.; Cala, A.R.; Rebecca, M.I.M.; Deanna, L.W.; Crawford, J.L.; Philippe, G.; Rose, J.K.C.; Viands, D.R.; et al. Season-long characterization of high-cannabinoid hemp (Cannabis sativa L.) reveals variation in cannabinoid accumulation, flowering time, and disease resistance. GCB Bioenergy 2021, 13, 546–561. [Google Scholar] [CrossRef] [Scilit]
- Andre, C.M.; Hausman, J.F.; Guerriero, G. Cannabis sativa: The plant of the thousand and one molecules. Front. Plant Sci. 2016, 7, 19. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Radwan, M.M.; Wanas, A.S.; Chandra, S.; Elsohly, M.A. Natural Cannabinoids of Cannabis and Methods of Analysis. In Cannabis sativa L.-Botany and Biotechnology; Chandra, S., Lata, H., Elsohly, A.M., Eds.; Springer International Publishing: Cham, Switzerland, 2017; pp. 161–181. [Google Scholar]
- Oppenheimer, D.G.; Herman, P.L.; Sivakumaran, S.; Esch, J.; Marks, M.D. A myb gene required for leaf trichome differentiation in Arabidopsis is expressed in stipules. Cell 1991, 67, 483–493. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Payne, C.T.; Zhang, F.; Lloyd, A.M. GL3 Encodes a bHLH Protein That Regulates Trichome Development in Arabidopsis Through Interaction With GL1 and TTG1. Genetics 2000, 156, 1349–1362. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Walker, A.R.; Davison, P.A.; Bolognesi-Winfield, A.C.; James, C.M.; Srinivasan, N.; Blundell, T.L.; Esch, J.J.; David Marks, M.; Gray, J.C. The TRANSPARENT TESTA GLABRA1 Locus, Which Regulates Trichome Differentiation and Anthocyanin Biosynthesis in Arabidopsis, Encodes a WD40 Repeat Protein. Plant Cell 1999, 11, 1337–1349. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Rerie, W.G.; Feldmann, K.A.; Marks, M.D. The GLABRA2 gene encodes a homeo domain protein required for normal trichome development in Arabidopsis. Genes Dev. 1994, 8, 1388–1399. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Szymanski, D.B.; Jilk, R.A.; Pollock, S.M.; Marks, M.D. Control of GL2 expression in Arabidopsis leaves and trichomes. Development 1998, 125, 1161–1171. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Schellmann, S.; Schnittger, A.; Kirik, V.; Wada, T.; Okada, K.; Beerman, A.; Thumfahrt, J.; Jürgens, G.; Hülskamp, M. TRIPTYCHON and CAPRICE mediate lateral inhibition during trichome and root hair patterning in Arabidopsis. EMBO J. 2002, 21, 5036–5046. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chalvin, C.; Drevensek, S.; Dron, M.; Bendahmane, A.; Boualem, A. Genetic Control of Glandular Trichome Development. Trends Plant Sci. 2020, 25, 477–487. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Han, G.; Li, Y.; Yang, Z.; Wang, C.; Zhang, Y.; Wang, B. Molecular Mechanisms of Plant Trichome Development. Front. Plant Sci. 2022, 13, 910228. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tian, N.; Liu, F.; Wang, P.; Zhang, X.; Li, X.; Wu, G. The molecular basis of glandular trichome development and secondary metabolism in plants. Plant Gene 2017, 12, 1–12. [Google Scholar] [CrossRef] [Scilit]
- Li, L.; Yu, S.; Chen, J.; Cheng, C.; Sun, J.; Xu, Y.; Deng, C.; Dai, Z.; Yang, Z.; Chen, X.; et al. Releasing the Full Potential of Cannabis through Biotechnology. Agronomy 2022, 12, 2439. [Google Scholar] [CrossRef] [Scilit]
- Pollio, A. The Name of Cannabis: A Short Guide for Nonbotanists. Cannabis Cannabinoid Res. 2016, 1, 234–238. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Livingston, S.J.; Quilichini, T.D.; Booth, J.K.; Wong, D.C.J.; Rensing, K.H.; Laflamme-Yonkman, J.; Castellarin, S.D.; Bohlmann, J.; Page, J.E.; Samuels, A.L. Cannabis glandular trichomes alter morphology and metabolite content during flower maturation. Plant J. 2020, 101, 37–56. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nolan, M.; Guo, Q.; Liu, L.; Dimopoulos, N.; Garcia-de Heer, L.; Barkla, B.J.; Kretzschmar, T. Characterisation of Cannabis glandular trichome development reveals distinct features of cannabinoid biosynthesis. Plant Cell Rep. 2025, 44, 30. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hülskamp, M.; Miséra, S.; Jürgens, G. Genetic dissection of trichome cell development in Arabidopsis. Cell 1994, 76, 555–566. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hancock, J.; Livingston, S.J.; Samuels, L. Building a biofactory: Constructing glandular trichomes in Cannabis sativa. Curr. Opin. Plant Biol. 2024, 80, 102549. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sutton, D.B.; Punja, Z.K.; Hamarneh, G. Characterization of trichome phenotypes to assess maturation and flower development in Cannabis sativa L. (Cannabis) by automatic trichome gland analysis. Smart Agric. Technol. 2023, 3, 100111. [Google Scholar] [CrossRef] [Scilit]
- Gjorgievska, V.S.; Karanfilova, I.C.; Trajkovska, A.; Karapandzova, M.; Petrovska, B.B.; Kulevanova, S.; Stefkov, G. Monitoring of Cannabis Cultivar Technological Maturity by Trichome Morphology Analysis and HPLC Phytocannabinoid Content. Pharmacogn. Res. 2022, 15, 94–100. [Google Scholar] [CrossRef] [Scilit]
- Huang, X.; Chen, W.; Zhao, Y.; Chen, J.; Ouyang, Y.; Li, M.; Gu, Y.; Wu, Q.; Cai, S.; Guo, F.; et al. Deep learning-based quantification and transcriptomic profiling reveal a methyl jasmonate-mediated glandular trichome formation pathway in Cannabis sativa. Plant J. 2024, 118, 1155–1173. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Small, E.; Naraine, S.G.U. Size matters: Evolution of large drug-secreting resin glands in elite pharmaceutical strains of Cannabis sativa (marijuana). Genet. Resour. Crop Evol. 2016, 63, 349–359. [Google Scholar] [CrossRef] [Scilit]
- Yang, C.; Sun, L.; Yasin, M.U.; Zulqarnain, H.; Ali, B.; Liu, Y.; Liu, B.; Gan, Y. GIS mediates GA signaling to directly target the expression of SPL15 to regulate trichome development in Arabidopsis thaliana. Plant Physiol. Biochem. 2025, 225, 109975. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yi, Y.; Zhu, M.; Gan, Y.; Liu, Y.; Cao, X. Ethylene regulates trichome initiation in Arabidopsis. Pak. J. Bot. 2026, 58, 1071–1077. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhou, Z.; Sun, L.; Zhao, Y.; An, L.; Yan, A.; Meng, X.; Gan, Y. Zinc Finger Protein 6 (ZFP6) regulates trichome initiation by integrating gibberellin and cytokinin signaling in Arabidopsis thaliana. New Phytol. 2013, 198, 699–708. [Google Scholar] [PubMed]
- Patra, B.; Pattanaik, S.; Yuan, L. Ubiquitin protein ligase 3 mediates the proteasomal degradation of GLABROUS 3 and ENHANCER of GLABROUS 3, regulators of trichome development and flavonoid biosynthesis in Arabidopsis. Plant J. 2013, 74, 435–447. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xue, X.Y.; Zhao, B.; Chao, L.M.; Chen, D.Y.; Cui, W.R.; Mao, Y.B.; Wang, L.J.; Chen, X.Y. Interaction between Two Timing MicroRNAs Controls Trichome Distribution in Arabidopsis. PLoS Genet. 2014, 10, e1004266. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yu, N.; Cai, W.J.; Wang, S.; Shan, C.M.; Wang, L.J.; Chena, X.Y. Temporal Control of Trichome Distribution by MicroRNA156-Targeted SPL Genes in Arabidopsis thaliana. Plant Cell 2010, 22, 2322–2335. [Google Scholar] [PubMed]
- Lian, H.; Wang, L.; Ma, N.; Zhou, C.M.; Han, L.; Zhang, T.Q.; Wang, J.W. Redundant and specific roles of individual MIR172 genes in plant development. PLoS Biol. 2021, 19, e3001044. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Vadde, B.V.L.; Challa, K.R.; Nath, U. The TCP4 transcription factor regulates trichome cell differentiation by directly activating GLABROUS INFLORESCENCE STEMS in Arabidopsis thaliana. Plant J. 2018, 93, 259–269. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hua, B.; Chang, J.; Wu, M.; Xu, Z.; Zhang, F.; Yang, M.; Xu, H.; Wang, L.J.; Chen, X.Y.; Wu, S. Mediation of JA signalling in glandular trichomes by the woolly/SlMYC1 regulatory module improves pest resistance in tomato. Plant Biotechnol. J. 2021, 19, 375–393. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yu, X.; Chen, G.; Tang, B.; Zhang, J.; Zhou, S.; Hu, Z. The Jasmonate ZIM-domain protein gene SlJAZ2 regulates plant morphology and accelerates flower initiation in Solanum lycopersicum plants. Plant Sci. 2018, 267, 65–73. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fonseca, R.; Capel, C.; Yuste-Lisbona, F.J.; Quispe, J.L.; Gómez-Martín, C.; Lebrón, R.; Hackenberg, M.; Oliver, J.L.; Angosto, T.; Lozano, R.; et al. Functional characterization of the tomato HAIRPLUS gene reveals the implication of the epigenome in the control of glandular trichome formation. Hortic. Res. 2022, 9, uhab015. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kim, S.M.; Choi, D.M.; Chun, J.I.; Kim, S.Y.; Kim, S.H.; Kim, J.I.; Jang, J.I.; Kim, K.; Park, S.J.; Seo, J.K.; et al. SlH3 and SlH4 promote multicellular trichome formation and elongation by upregulating Woolly in tomato. Hortic. Res. 2025, 12, uhaf008. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zheng, F.; Cui, L.; Li, C.; Xie, Q.; Ai, G.; Wang, J.; Yu, H.; Wang, T.; Zhang, J.; Ye, Z.; et al. Hair interacts with SlZFP8-like to regulate the initiation and elongation of trichomes by modulating SlZFP6 expression in tomato. J. Exp. Bot. 2022, 73, 228–244. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gao, S.; Gao, Y.; Xiong, C.; Yu, G.; Chang, J.; Yang, Q.; Yang, C.; Ye, Z. The tomato B-type cyclin gene, SlCycB2, plays key roles in reproductive organ development, trichome initiation, terpenoids biosynthesis and Prodenia litura defense. Plant Sci. 2017, 262, 103–114. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yang, C.; Li, H.; Zhang, J.; Wang, T.; Ye, Z. Fine-mapping of the woolly gene controlling multicellular trichome formation and embryonic development in tomato. Theor. Appl. Genet. 2011, 123, 625–633. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xu, J.; Van Herwijnen, Z.O.; Dräger, D.B.; Sui, C.; Haring, M.A.; Schuurink, R.C. SlMYC1 regulates type VI glandular trichome formation and terpene biosynthesis in tomato glandular cells. Plant Cell 2018, 30, 2988–3005. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Shi, Y.; Wang, Y.; Pan, Y.; Deng, C.; Zeng, T.; Su, D.; Lu, W.; Lin, Y.; Han, J.; Deng, W.; et al. The SlGRAS9-SlMYC1 regulatory module controls glandular trichome formation and modulates resilience to pest in tomato. Plant J. 2025, 122, e70183. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Qi, T.; Wu, M.; Wang, S.; Yuan, Y.; Xu, X.; Zhang, Q.; Jian, Y.; Qiu, D.; Cheng, Y.; Huang, B.; et al. SlMYB72 and SlMYB75 antagonistically regulate trichome formation via the MYB-bHLH-WD40 complex in tomato. J. Biol. Chem. 2025, 301, 108313. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Matías-Hernández, L.; Jiang, W.; Yang, K.; Tang, K.; Brodelius, P.E.; Pelaz, S. AaMYB1 and its orthologue AtMYB61 affect terpene metabolism and trichome development in Artemisia annua and Arabidopsis thaliana. Plant J. 2017, 90, 520–534. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Shi, P.; Fu, X.; Shen, Q.; Liu, M.; Pan, Q.; Tang, Y.; Jiang, W.; Lv, Z.; Yan, T.; Ma, Y.; et al. The roles of AaMIXTA1 in regulating the initiation of glandular trichomes and cuticle biosynthesis in Artemisia annua. New Phytol. 2018, 217, 261–276. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yan, T.; Chen, M.; Shen, Q.; Li, L.; Fu, X.; Pan, Q.; Tang, Y.; Shi, P.; Lv, Z.; Jiang, W.; et al. HOMEODOMAIN PROTEIN 1 is required for jasmonate-mediated glandular trichome initiation in Artemisia annua. New Phytol. 2017, 213, 1145–1155. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yan, T.; Li, L.; Xie, L.; Chen, M.; Shen, Q.; Pan, Q.; Fu, X.; Shi, P.; Tang, Y.; Huang, H.; et al. A novel HD-ZIP IV/MIXTA complex promotes glandular trichome initiation and cuticle development in Artemisia annua. New Phytol. 2018, 218, 567–578. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Maes, L.; Van Nieuwerburgh, F.C.W.; Zhang, Y.; Reed, D.W.; Pollier, J.; Vande Casteele, S.R.F.; Inzé, D.; Covello, P.S.; Deforce, D.L.D.; Goossens, A. Dissection of the phytohormonal regulation of trichome formation and biosynthesis of the antimalarial compound artemisinin in Artemisia annua plants. New Phytol. 2011, 189, 176–189. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hu, X.; Liu, H.; Chen, T.; Ye, Y.; Shao, J.; Yan, X.; Peng, B.; Li, L.; Tang, K. AaPDF2 promotes glandular trichome formation in Artemisia annua through jasmonic acid signaling. Ind. Crops Prod. 2025, 234, 121630. [Google Scholar] [CrossRef] [Scilit]
- Zhang, M.; Li, M.; An, Y.; Liu, C.; Zhao, Q.; Zhang, D.; Pan, B.; Tan, H. Single-nucleus transcriptomics reveal the morphogenesis and artemisinin biosynthesis in Artemisia annua glandular trichomes. Nat. Commun. 2025, 16, 8646. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, C.; Chen, T.; Li, Y.; Liu, H.; Qin, W.; Wu, Z.; Peng, B.; Wang, X.; Yan, X.; Fu, X.; et al. AaWIN1, an AP2/ERF protein, positively regulates glandular secretory trichome initiation in Artemisia annua. Plant Sci. 2023, 329, 111602. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dong, B.; Wang, X.; Jiang, R.; Fang, S.; Li, J.; Li, Q.; Lv, Z.Y.; Chen, W.S. AaCycTL Regulates Cuticle and Trichome Development in Arabidopsis and Artemisia annua L. Front. Plant Sci. 2021, 12, 808283. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xie, L.; Yan, T.; Li, L.; Chen, M.; Hassani, D.; Li, Y.; Qin, W.; Liu, H.; Chen, T.; Fu, X.; et al. An HD-ZIP-MYB complex regulates glandular secretory trichome initiation in Artemisia annua. New Phytol. 2021, 231, 2050–2064. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xie, L.; Yan, T.; Li, L.; Chen, M.; Ma, Y.; Hao, X.; Fu, X.; Shen, Q.; Huang, Y.; Qin, W.; et al. The WRKY transcription factor AaGSW2 promotes glandular trichome initiation in Artemisia annua. J. Exp. Bot. 2021, 72, 1691–1701. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- He, Y.; Fu, X.; Li, L.; Sun, X.; Tang, K.; Zhao, J. AaSPL9 affects glandular trichomes initiation by positively regulating expression of AaHD1 in Artemisia annua L. Plant Sci. 2022, 317, 111172. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ahmad Khan, R.; Mohammad; Kumar, A.; Abbas, N. AaGL3-like is jasmonate-induced bHLH transcription factor that positively regulates trichome density in Artemisia annua. Gene 2024, 904, 148213. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jiang, R.; Chen, W.; Li, Q.; Guo, J.; Lv, Z.; Chen, W. Genome-wide identification of the WD40 protein family and functional characterization of AaTTG1 in Artemisia annua. Int. J. Biol. Macromol. 2025, 289, 138834. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, Z.; Yan, X.; Zhang, H.; Meng, Y.; Pan, Y.; Cui, H. NtCycB2 negatively regulates tobacco glandular trichome formation, exudate accumulation, and aphid resistance. Plant Mol. Biol. 2022, 108, 65–76. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, Y.; Liu, D.; Khan, A.R.; Liu, B.; Wu, M.; Huang, L.; Wu, J.; Song, G.; Ni, H.; Ying, H.; et al. NbGIS regulates glandular trichome initiation through GA signaling in tobacco. Plant Mol. Biol. 2018, 98, 153–167. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, H.; Li, W.; Niu, D.; Wang, Z.; Yan, X.; Yang, X.; Yang, Y.; Cui, H. Tobacco transcription repressors NtJAZ: Potential involvement in abiotic stress response and glandular trichome induction. Plant Physiol. Biochem. 2019, 141, 388–397. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Suárez-Baron, H.; Alzate, J.F.; González, F.; Pelaz, S.; Ambrose, B.A.; Pabón-Mora, N. Gene expression underlying floral epidermal specialization in Aristolochia fimbriata (Aristolochiaceae). Ann. Bot. 2021, 127, 749–764. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Peng, C.; Yao, X.; Fu, X.; Lyu, S.; Yuan, Y.; Liao, H.; Yin, X.; Cheng, J.; Li, X.; Kong, H.; et al. Evolution of short trichomes and long hairs on Nigella petals through co-option of bHLH and non-MIXTA MYB genes. Nat. Commun. 2025, 16, 8304. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kirik, V.; Simon, M.; Huelskamp, M.; Schiefelbein, J. The ENHANCER OF TRY AND CPC1 gene acts redundantly with TRIPTYCHON and CAPRICE in trichome and root hair cell patterning in Arabidopsis. Dev. Biol. 2004, 268, 506–513. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wada, T.; Tachibana, T.; Shimura, Y.; Okada, K. Epidermal cell differentiation in Arabidopsis determined by a Myb homolog, CPC. Science 1997, 277, 1113–1116. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Khosla, A.; Paper, J.M.; Boehler, A.P.; Bradley, A.M.; Neumann, T.R.; Schrick, K. HD-Zip proteins GL2 and HDG11 have redundant functions in Arabidopsis trichomes, and GL2 activates a positive feedback loop via MYB23. Plant Cell 2014, 26, 2184–2200. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Arteaga, N.; Méndez-Vigo, B.; Fuster-Pons, A.; Savic, M.; Murillo-Sánchez, A.; Picó, F.X.; Alonso-Blanco, C. Differential environmental and genomic architectures shape the natural diversity for trichome patterning and morphology in different Arabidopsis organs. Plant Cell Environ. 2022, 45, 3018–3035. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Méndez-Vigo, B.; Arteaga, N.; Murillo-Sánchez, A.; Alba, S.; Alonso-Blanco, C. The bHLH transcription factor gene EGL3 accounts for the natural diversity in Arabidopsis fruit trichome pattern and morphology. Plant Physiol. 2025, 197, kiae673. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Symonds, V.V.; Hatlestad, G.; Lloyd, A.M. Natural allelic variation defines a role for ATMYC1: Trichome cell fate determination. PLoS Genet. 2011, 7, e1002069. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fambrini, M.; Pugliesi, C. The Dynamic Genetic-Hormonal Regulatory Network Controlling the Trichome Development in Leaves. Plants 2019, 8, 253. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, X.; Yan, F.; Tang, Y.; Yuan, Y.; Deng, W.; Li, Z. Auxin Response Gene SlARF3 Plays Multiple Roles in Tomato Development and is Involved in the Formation of Epidermal Cells and Trichomes. Plant Cell Physiol. 2015, 56, 2110–2124. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Galdon-Armero, J.; Arce-Rodriguez, L.; Downie, M.; Li, J.; Martin, C. A scanning electron micrograph-based resource for identification of loci involved in epidermal development in Tomato: Elucidation of a new function for the mixta-like transcription factor in Leaves. Plant Cell 2020, 32, 1414–1433. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Davis, G.V.; Glover, B.J. Characterisation of the R2R3 Myb subgroup 9 family of transcription factors in tomato. PLoS ONE 2024, 19, e0295445. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ying, S.; Su, M.; Wu, Y.; Zhou, L.; Fu, R.; Li, Y.; Guo, H.; Luo, J.; Wang, S.; Zhang, Y. Trichome regulator SlMIXTA-like directly manipulates primary metabolism in tomato fruit. Plant Biotechnol. J. 2020, 18, 354–363. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nadakuduti, S.S.; Pollard, M.; Kosma, D.K.; Allen, C.; Ohlrogge, J.B.; Barry, C.S. Pleiotropic phenotypes of the sticky peel mutant provide new insight into the role of CUTIN DEFICIENT2 in epidermal cell function in tomato. Plant Physiol. 2012, 159, 945–960. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yuan, M.; Sheng, Y.; Bao, J.; Wu, W.; Nie, G.; Wang, L.; Cao, J. AaMYC3 bridges the regulation of glandular trichome density and artemisinin biosynthesis in Artemisia annua. Plant Biotechnol. J. 2025, 23, 315–332. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lv, Z.; Li, J.X.; Qiu, S.; Qi, F.; Su, H.; Bu, Q.; Jiang, R.; Tang, K.; Zhang, L.; Chen, W. The transcription factors TLR1 and TLR2 negatively regulate trichome density and artemisinin levels in Artemisia annua. J. Integr. Plant Biol. 2022, 64, 1212–1228. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Qin, W.; Xie, L.; Li, Y.; Liu, H.; Fu, X.; Chen, T.; Hassani, D.; Li, L.; Sun, X.; Tang, K. An R2R3-MYB Transcription Factor Positively Regulates the Glandular Secretory Trichome Initiation in Artemisia annua L. Front. Plant Sci. 2021, 12, 657156. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhou, Z.; Tan, H.; Li, Q.; Li, Q.; Wang, Y.; Bu, Q.; Li, Y.; Wu, Y.; Chen, W.; Zhang, L. TRICHOME AND ARTEMISININ REGULATOR 2 positively regulates trichome development and artemisinin biosynthesis in Artemisia annua. New Phytol. 2020, 228, 932–945. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, T.T.; Liu, H.; Li, Y.P.; Yao, X.H.; Qin, W.; Yan, X.; Wang, X.Y.; Peng, B.W.; Zhang, Y.J.; Shao, J.; et al. AaSEPALLATA1 integrates jasmonate and light-regulated glandular secretory trichome initiation in Artemisia annua. Plant Physiol. 2023, 192, 1483–1497. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, H.; He, W.; Yao, X.; Yan, X.; Wang, X.; Peng, B.; Zhang, Y.; Shao, J.; Hu, X.; Miao, Q.; et al. The Light- and Jasmonic Acid-Induced AaMYB108-like Positive Regulates the Initiation of Glandular Secretory Trichome in Artemisia annua L. Int. J. Mol. Sci. 2023, 24, 12929. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Khan, R.A.; Kumar, A.; Abbas, N. A bHLH transcription factor AaMYC2-type positively regulates glandular trichome density and artemisinin biosynthesis in Artemisia annua. Physiol. Plant. 2024, 176, e14581. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fu, X.; Zheng, H.; Wang, Y.; Liu, H.; Liu, P.; Li, L.; Zhao, J.; Sun, X.; Tang, K. AaABCG20 transporter involved in cutin and wax secretion affects the initiation and development of glandular trichomes in Artemisia annua. Plant Sci. 2024, 339, 111959. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Suárez-Baron, H.; Alzate, J.F.; Ambrose, B.A.; Pelaz, S.; González, F.; Pabón-Mora, N. Comparative morphoanatomy and transcriptomic analyses reveal key factors controlling floral trichome development in Aristolochia (Aristolochiaceae). J. Exp. Bot. 2023, 74, 6588–6607. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Suárez-Baron, H.; Alzate, J.F.; González, F.; Ambrose, B.A.; Pabón-Mora, N. Genetic mechanisms underlying perianth epidermal elaboration of Aristolochia ringens Vahl (Aristolochiaceae). Flora Morphol. Distrib. Funct. Ecol. Plants 2019, 253, 56–66. [Google Scholar] [CrossRef] [Scilit]
- Liu, R.; Wang, Y.; Tang, S.; Cai, J.; Liu, S.; Zheng, P.; Sun, B. Genome-wide identification of the tea plant bHLH transcription factor family and discovery of candidate regulators of trichome formation. Sci. Rep. 2021, 11, 10764. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zheng, J.; Wu, Y.; Zhang, L.; Yang, L.; Jin, J.; Li, C.; Tong, S.; Yu, J. Overexpression of NtMYB306c reduces the glandular trichomes density in tobacco. Biochem. Biophys. Res. Commun. 2025, 772, 152061. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bai, Y.; Xu, Y.; Qi, X.; Li, L.; Yu, X.; Fang, H.; Liu, D.; Chen, F.; Liang, C. Overexpression of the Mentha canadensis McTTG2 gene positively regulates trichome development and proanthocyanidins biosynthesis in transgenic Arabidopsis. Plant Sci. 2026, 366, 113065. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kasili, R.; Walker, J.D.; Simmons, L.A.; Zhou, J.; De Veylder, L.; Larkin, J.C. SIAMESE Cooperates With the CDH1-like Protein CCS52A1 to Establish Endoreplication in Arabidopsis thaliana Trichomes. Genetics 2010, 185, 257–268. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sugimoto-Shirasu, K.; Stacey, N.J.; Corsar, J.; Roberts, K.; McCann, M.C. DNA topoisomerase VI is essential for endoreduplication in Arabidopsis. Curr. Biol. 2002, 12, 1782–1786. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, H.; Fowke, L.C.; Crosby, W.L. A plant cyclin-dependent kinase inhibitor gene. Nature 1997, 386, 451–452. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, L.; Wang, Y.; Cao, W.; Yang, L.; Zhang, C.; Yuan, L.; Wang, D.; Wang, W.; Zhang, H.; Schiefelbein, J.; et al. TRANSPARENT TESTA GLABRA2 defines trichome cell shape by modulating actin cytoskeleton in Arabidopsis thaliana. Plant Physiol. 2024, 195, 1256–1276. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Luo, D.; Oppenheimer, D.G. Genetic control of trichome branch number in Arabidopsis: The roles of the FURCA loci. Development 1999, 126, 5547–5557. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xie, W.; Zhao, Y.; Deng, X.; Chen, R.; Qiang, Z.; García-Caparros, P.; Mao, T.; Qin, T. GLABRA3-mediated trichome branching requires transcriptional repression of MICROTUBULE-DESTABILIZING PROTEIN25. Plant Physiol. 2025, 197, kiae563. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Folkers, U.; Kirik, V.; Schöbinger, U.; Falk, S.; Krishnakumar, S.; Pollock, M.A.; Oppenheimer, D.G.; Day, I.; Reddy, A.R.; Jürgens, G.; et al. The cell morphogenesis gene ANGUSTIFOLIA encodes a CtBP/BARS-like protein and is involved in the control of the microtubule cytoskeleton. EMBO J. 2002, 21, 1280–1288. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Oppenheimer, D.G.; Pollock, M.A.; Vacik, J.; Szymanski, D.B.; Ericson, B.; Feldmann, K.; Marks, M.D. Essential role of a kinesin-like protein in Arabidopsis trichome morphogenesis. Proc. Natl. Acad. Sci. USA 1997, 94, 6261–6266. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ilgenfritz, H.; Bouyer, D.; Schnittger, A.; Mathur, J.; Kirik, V.; Schwab, B.; Chua, N.H.; Jürgens, G.; Hülskamp, M. The Arabidopsis STICHEL gene is a regulator of trichome branch number and encodes a novel protein. Plant Physiol. 2003, 131, 643–655. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nakamura, M.; Katsumata, H.; Abe, M.; Yabe, N.; Komeda, Y.; Yamamoto, K.T.; Takahashi, T. Characterization of the class IV homeodomain-Leucine zipper gene family in Arabidopsis. Plant Physiol. 2006, 141, 1363–1375. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, S.F.; Milliken, O.N.; Pham, H.; Seyit, R.; Napoli, R.; Preston, J.; Koltunow, A.M.; Parish, R.W. The Arabidopsis MYB5 transcription factor regulates mucilage synthesis, seed coat development, and trichome morphogenesis. Plant Cell 2009, 21, 72–89. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chun, J.-I.; Kim, S.-M.; Kim, H.; Cho, J.-Y.; Kwon, H.-W.; Kim, J.-I.; Seo, J.-K.; Jung, C.; Kang, J.-H. SlHair2 Regulates the Initiation and Elongation of Type I Trichomes on Tomato Leaves and Stems. Plant Cell Physiol. 2021, 9, 1446–1459. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, R.; Wang, X.; Zhang, S.; Liu, X.; Zhou, Z.; Liu, Z.; Wang, K.; Tian, Y.; Wang, H.; Zhang, Y.; et al. Two zinc-finger proteins control the initiation and elongation of long stalk trichomes in tomato. J. Genet. Genom. 2021, 48, 1057–1069. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xie, Q.; Gao, Y.; Li, J.; Yang, Q.; Qu, X.; Li, H.; Zhang, J.; Wang, T.; Ye, Z.; Yang, C. The HD-Zip IV transcription factor SlHDZIV8 controls multicellular trichome morphology by regulating the expression of Hairless-2. J. Exp. Bot. 2020, 71, 7132–7145. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zocca, P.; van Doore, E.; Roovers, A.J.M.; Glas, J.J.; Uittenbogaard, M.; Verlaan, M.G.; van Herwijnen, Z.; Haring, M.A.; Schuurink, R.C. Glandless, a tomato HD-ZIP transcription factor, is important for the gland formation of type VI trichomes. Plant J. 2025, 123, e70308. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tan, H.; Xiao, L.; Gao, S.; Li, Q.; Chen, J.; Xiao, Y.; Ji, Q.; Chen, R.; Chen, W.; Zhang, L. TRICHOME and ARTEMISININ REGULATOR 1 is required for trichome development and artemisinin biosynthesis in Artemisia annua. Mol. Plant 2015, 8, 1396–1411. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hao, X.; Zhong, Y.; Fu, X.; Lv, Z.; Shen, Q.; Yan, T.; Shi, P.; Ma, Y.; Chen, M.; Lv, X.; et al. Transcriptome analysis of genes associated with the artemisinin biosynthesis by jasmonic acid treatment under the light in artemisia annua. Front. Plant Sci. 2017, 8, 971. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ma, D.; Pu, G.; Lei, C.; Ma, L.; Wang, H.; Guo, Y.; Chen, J.; Du, Z.; Wang, H.; Li, G.; et al. Isolation and characterization of AaWRKY1, an artemisia annua transcription factor that regulates the amorpha-4,11-diene synthase gene, a key gene of artemisinin biosynthesis. Plant Cell Physiol. 2009, 50, 2146–2161. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Janga, M.R.; Pandeya, D.; Campbell, L.A.M.; Konganti, K.; Villafuerte, S.T.; Puckhaber, L.; Pepper, A.; Stipanovic, R.D.; Scheffler, J.A.; Rathore, K.S. Genes regulating gland development in the cotton plant. Plant Biotechnol. J. 2019, 17, 1142–1153. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dai, Y.; Liu, S.; Zuo, D.; Wang, Q.; Lv, L.; Zhang, Y.; Cheng, H.; Yu, J.Z.; Song, G. Identification of MYB gene family and functional analysis of GhMYB4 in cotton (Gossypium spp.). Mol. Genet. Genom. 2023, 298, 755–766. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, Y.; Wang, D.; Li, H.; Bai, H.; Sun, M.; Shi, L. Formation mechanism of glandular trichomes involved in the synthesis and storage of terpenoids in lavender. BMC Plant Biol. 2023, 23, 307. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dong, M.; Xue, S.; Bartholomew, E.S.; Zhai, X.; Sun, L.; Xu, S.; Zhang, Y.; Yin, S.; Ma, W.; Chen, S.; et al. Transcriptomic and functional analysis provides molecular insights into multicellular trichome development. Plant Physiol. 2022, 189, 301–314. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Feng, Z.; Sun, L.; Dong, M.; Fan, S.; Shi, K.; Qu, Y.; Zhu, L.; Shi, J.; Wang, W.; Liu, Y.; et al. Identification and Functional Characterization of CsMYCs in Cucumber Glandular Trichome Development. Int. J. Mol. Sci. 2023, 24, 6435. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, Y.; Yan, M.; Lan, H. Regulation of trichome formation by phytohormones and cytoskeleton genes in Salsola ferganica, an annual desert halophyte. Plant Sci. 2026, 362, 112861. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bassolino, L.; Buti, M.; Fulvio, F.; Pennesi, A.; Mandolino, G.; Milc, J.; Francia, E.; Paris, R. In silico identification of myb and bhlh families reveals candidate transcription factors for secondary metabolic pathways in Cannabis sativa L. Plants 2020, 9, 1540. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, Y.; Zhu, P.; Cai, S.; Haughn, G.; Page, J.E. Three novel transcription factors involved in cannabinoid biosynthesis in Cannabis sativa L. Plant Mol. Biol. 2021, 106, 49–65. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ma, G.; Zelman, A.K.; Apicella, P.V.; Berkowitz, G. Genome-Wide Identification and Expression Analysis of Homeodomain Leucine Zipper Subfamily IV (HD-ZIP IV) Gene Family in Cannabis sativa L. Plants 2022, 11, 1307. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Haiden, S.R.; Apicella, P.V.; Ma, Y.; Berkowitz, G.A. Overexpression of CsMIXTA, a Transcription Factor from Cannabis sativa, Increases Glandular Trichome Density in Tobacco Leaves. Plants 2022, 11, 1519. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Del Rosario-Makridis, G.N. Molecular Regulation of Glandular Trichome Initiation and Morphogenesis in Cannabis sativa L. Ph.D. Thesis, La Trobe University, Melbourne, Australia, 2023. [Google Scholar]
- Conneely, L.J.; Hurgobin, B.; Ng, S.; Tamiru-Oli, M.; Lewsey, M.G. Characterization of the Cannabis sativa glandular trichome epigenome. BMC Plant Biol. 2024, 24, 1075. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Siazon, P.M.; Nolan, M.; Guo, Q.; Perovich, R.; Kretzschmar, T.; Mieog, J.C. Heads Up: Transcriptomics Reveal Functional Roles of Cannabis Glandular Trichome Stalks. Plants 2026, 15, 1624. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhu, X.; Mi, Y.; Cao, X.; Chen, W.; Fan, P.; Wang, J.; Zhang, Y.; Yang, W.; Wan, H.; Chen, S.; et al. A Novel CsYABBY3-CsAS1 Feedback Loop Coordinates Trichome Differentiation and Cannabinoid Biosynthesis in Cannabis sativa L. Adv. Sci. 2026, 13, e75055. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tamiru-Oli, M.; Hurgobin, B.; Berkowitz, O.; Yin, L.; Jost, R.; Gvaramiya, S.; Welling, M.; Doblin, M.S.; Bacic, A.; Whelan, J.; et al. Insights into glandular trichome biology from analysis of organ-specific gene expression programmes in Cannabis, hop and tomato. Plant J. 2026, 125, e70774. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tanney, C.A.S.; Backer, R.; Geitmann, A.; Smith, D.L. Cannabis Glandular Trichomes: A Cellular Metabolite Factory. Front. Plant Sci. 2021, 12, 721986. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Welling, M.T.; Liu, L.; Shapter, T.; Raymond, C.A.; King, G.J. Characterisation of cannabinoid composition in a diverse Cannabis sativa L. germplasm collection. Euphytica 2016, 208, 463–475. [Google Scholar] [CrossRef] [Scilit]
- Braich, S.; Baillie, R.C.; Jewell, L.S.; Spangenberg, G.C.; Cogan, N.O.I. Generation of a Comprehensive Transcriptome Atlas and Transcriptome Dynamics in Medicinal Cannabis. Sci. Rep. 2019, 9, 16583. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yeo, H.C.; Reddy, V.A.; Mun, B.G.; Leong, S.H.; Dhandapani, S.; Rajani, S.; Jang, I.C. Comparative Transcriptome Analysis Reveals Coordinated Transcriptional Regulation of Central and Secondary Metabolism in the Trichomes of Cannabis Cultivars. Int. J. Mol. Sci. 2022, 23, 8310. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Conneely, L.J.; Mauleon, R.; Mieog, J.; Barkla, B.J.; Kretzschmar, T. Characterization of the Cannabis sativa glandular trichome proteome. PLoS ONE 2021, 16, e0242633. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Brenneisen, R. Chemistry and analysis of phytocannabinoids and other Cannabis constituents. In Marijuana and the Cannabinoids; Mahmoud, A., Ed.; Humana Press: Totowa, NJ, USA, 2007; pp. 17–49. [Google Scholar]
- Sirikantaramas, S.; Taura, F. Cannabinoids: Biosynthesis and Biotechnological Applications. In Cannabis sativa L.-Botany and Biotechnology; Chandra, S., Lata, H., ElSohly, M., Eds.; Springer International Publishing: Cham, Switzerland, 2017; pp. 183–206. [Google Scholar]
- Taura, F.; Sirikantaramas, S.; Shoyama, Y.; Yoshikai, K.; Shoyama, Y.; Morimoto, S. Cannabidiolic-acid synthase, the chemotype-determining enzyme in the fiber-type Cannabis sativa. FEBS Lett. 2007, 581, 2929–2934. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Aizpurua-Olaizola, O.; Soydaner, U.; Öztürk, E.; Schibano, D.; Simsir, Y.; Navarro, P.; Etxebarria, N.; Usobiaga, A. Evolution of the Cannabinoid and Terpene Content during the Growth of Cannabis sativa Plants from Different Chemotypes. J. Nat. Prod. 2016, 79, 324–331. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Booth, J.K.; Bohlmann, J. Terpenes in Cannabis sativa—From plant genome to humans. Plant Sci. 2019, 284, 67–72. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Desaulniers Brousseau, V.; Wu, B.S.; MacPherson, S.; Morello, V.; Lefsrud, M. Cannabinoids and Terpenes: How Production of Photo-Protectants Can Be Manipulated to Enhance Cannabis sativa L. Phytochemistry. Front. Plant Sci. 2021, 12, 2021. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ferri, E.; Cerrato, A.; Caprari, C.; Russo, F.; Laganà, A.; Capriotti, A.L.; Faggiana, G.; Moro, A.; Citti, C.; Cannazza, G. Single trichome phytocannabinomics of two different Cannabis varieties. J. Pharm. Biomed. Anal. 2025, 261, 116836. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Schachtsiek, J.; Hussain, T.; Azzouhri, K.; Kayser, O.; Stehle, F. Virus-induced gene silencing (VIGS) in Cannabis sativa L. Plant Methods 2019, 15, 157. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zager, J.J.; Lange, I.; Srividya, N.; Smith, A.; Markus Lange, B. Gene networks underlying cannabinoid and terpenoid accumulation in Cannabis. Plant Physiol. 2019, 180, 1877–1897. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Deguchi, M.; Bogush, D.; Weeden, H.; Spuhler, Z.; Potlakayala, S.; Kondo, T.; Zhang, Z.J.; Rudrabhatla, S. Establishment and optimization of a hemp (Cannabis sativa L.) agroinfiltration system for gene expression and silencing studies. Sci. Rep. 2020, 10, 3504. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, X.; Xu, G.; Cheng, C.; Lei, L.; Sun, J.; Xu, Y.; Deng, C.; Dai, Z.; Yang, Z.; Chen, X.; et al. Establishment of an Agrobacterium-mediated genetic transformation and CRISPR/Cas9-mediated targeted mutagenesis in Hemp (Cannabis sativa L.). Plant Biotechnol. J. 2021, 19, 1979–1987. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, M.; Wu, Q.; Guo, F.; Ouyang, Y.; Ao, D.; You, S.; Liu, Y. A versatile, rapid Agrobacterium-mediated transient expression system for functional genomics studies in Cannabis seedling. Planta 2024, 260, 18. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Beard, K.M.; Boling, A.W.H.; Bargmann, B.O.R. Industrial Crops & Products Protoplast isolation, transient transformation, and flow-cytometric analysis of reporter-gene activation in Cannabis sativa L. Ind. Crops Prod. 2021, 164, 113360. [Google Scholar]
- Matchett-Oates, L.; Mohamaden, E.; Spangenberg, G.C.; Cogan, N.O.I. Development of a robust transient expression screening system in protoplasts of Cannabis. Vitr. Cell. Dev. Biol. Plant 2021, 57, 1040–1050. [Google Scholar] [CrossRef] [Scilit]
- Kim, A.L.; Yun, Y.J.; Choi, H.W.; Hong, C.H.; Shim, H.J.; Lee, J.H.; Kim, Y.C. Establishment of efficient Cannabis (Cannabis sativa L.) protoplast isolation and transient expression condition. Plant Biotechnol. Rep. 2022, 16, 613–619. [Google Scholar] [CrossRef] [Scilit]
- Stelmach-Wityk, K.; Szymonik, K.; Jones, A.M.P.; Grzebelus, E. A novel protocol for protoplast isolation, transfection, and culture in Cannabis sativa L. BMC Plant Biol. 2025, 25, 1629. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fousek, J.; Dusek, J.; Hoffmeisterová, H.; Cerovska, N.; Kundu, K.J.; Moravec, T. Quantitative Estimation of Promoter Activity in Cannabis sativa Using Agroinfiltration-Based Transient Gene Expression. In Plant Functional Genomics: Methods and Protocols, Methods in Molecular Biology; Maghuly, F., Ed.; Springer Science+Business Media: Vienna, Austria, 2024; Volume 1, pp. 245–253. [Google Scholar]
- Schilling, S.; Dowling, C.A.; Shi, J.; Ryan, L.; Hunt, D.J.L.; O’Reilly, E.; Perry, A.S.; Kinnane, O.; McCabe, P.F.; Melzer, R. The Cream of the Crop: Biology, Breeding and Applications of Cannabis sativa. Annu. Plant Rev. Online 2020, 4, 471–528. [Google Scholar]
- Wu, M.; Chang, J.; Han, X.; Shen, J.; Yang, L.; Hu, S.; Huang, B.B.; Xu, H.; Xu, M.; Wu, S.; et al. A HD-ZIP transcription factor specifies fates of multicellular trichomes via dosage-dependent mechanisms in tomato. Dev. Cell 2023, 58, 278–288.e5. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wu, M.L.; Bian, X.X.; Hu, S.R.; Huang, B.B.; Shen, J.Y.; Du, Y.D.; Wang, Y.L.; Xu, M.Y.; Xu, H.M.; Yang, M.N.; et al. A gradient of the HD-Zip regulator Woolly regulates multicellular trichome morphogenesis in tomato. Plant Cell 2024, 36, 2375–2392. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yin, M.; Pan, G.; Tao, J.; Doblin, M.S.; Zeng, W.; Pan, L.; Zhao, L.; Li, Z.; Jiang, H.; Chang, L.; et al. Identification of MYB genes reveals their potential functions in cadmium stress response and the regulation of cannabinoid biosynthesis in hemp. Ind. Crops Prod. 2022, 180, 114607. [Google Scholar] [CrossRef] [Scilit]
- De Meijer, E.P.M.; Hammond, K.M. The inheritance of chemical phenotype in Cannabis sativa L. (V): Regulation of the propyl-/pentyl cannabinoid ratio, completion of a genetic model. Euphytica 2016, 210, 291–307. [Google Scholar] [CrossRef] [Scilit]
- De Meijer, E.P.M.; Hammond, K.M.; Sutton, A. The inheritance of chemical phenotype in Cannabis sativa L. (IV): Cannabinoid-free plants. Euphytica 2009, 168, 95–112. [Google Scholar] [CrossRef] [Scilit]
- Onofri, C.; De Meijer, E.P.M.; Mandolino, G. Sequence heterogeneity of cannabidiolic- and tetrahydrocannabinolic acid-synthase in Cannabis sativa L. and its relationship with chemical phenotype. Phytochemistry 2015, 116, 57–68. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cascini, F.; Farcomeni, A.; Migliorini, D.; Baldassarri, L.; Boschi, I.; Martello, S.; Amaducci, S.; Lucini, L.; Bernardi, J. Highly predictive genetic markers distinguish drug-type from fiber-type Cannabis sativa L. Plants 2019, 8, 496. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fulvio, F.; Paris, R.; Montanari, M.; Citti, C.; Cilento, V.; Bassolino, L.; Moschella, A.; Alberti, I.; Pecchioni, N.; Cannazza, G.; et al. Analysis of sequence variability and transcriptional profile of cannabinoid synthase genes in Cannabis sativa l. Chemotypes with a focus on cannabichromenic acid synthase. Plants 2021, 10, 1857. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sayre, R.; Soto-Aguilar, M.; Zidenga, T.; Carvalho, E. Systems and Methods for Enhancing Trichome Formation and Density in Cannabis. U.S. Patent 10724048B2, 28 July 2020. [Google Scholar]
- Sayre, R.; Soto-Aguilar, M.; Zidenga, T.; Carvalho, E. Systems and Methods for Enhancing Trichome Formation and Density in Cannabis. U.S. Patent 20190352662A1, 21 November 2019. [Google Scholar]
- Sayre, R.; Zidenga, T.; Goncalves, E. Systems and Methods for Enhancing Trichome Formation and Density in Cannabis. WO2019147873A2, 1 August 2019. [Google Scholar]
- Li, J.; Wang, X.; Jiang, R.; Dong, B.; Fang, S.; Li, Q.; Lv, Z.; Chen, W. Phytohormone-Based Regulation of Trichome Development. Front Plant Sci. 2021, 12, 734776. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dimopoulos, N.; Guo, Q.; Liu, L.; Nolan, M.; Das, R.; Garcia-de Heer, L.; Mieog, J.C.; Barkla, B.J.; Kretzschmar, T. An In Vitro Phytohormone Survey Reveals Concerted Regulation of the Cannabis Glandular Trichome Disc Cell Proteome. Plants 2025, 14, 694. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Flores-Sanchez, I.J.; Pec, J.; Fei, J.; Choi, Y.H.; Dusek, J.; Verpoorte, R. Elicitation studies in cell suspension cultures of Cannabis sativa L. J. Biotechnol. 2009, 143, 157–168. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Backer, R.; Mandolino, G.; Wilkins, O.; Elsohly, M.A.; Smith, D.L. Editorial: Cannabis Genomics, Breeding and Production. Front. Plant Sci. 2020, 11, 591445. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ingvardsen, C.R.; Brinch-Pedersen, H. Challenges and potentials of new breeding techniques in Cannabis sativa. Front. Plant Sci. 2023, 14, 1154332. [Google Scholar] [CrossRef] [Scilit] [PubMed]
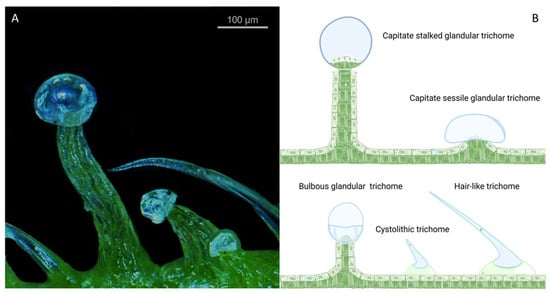
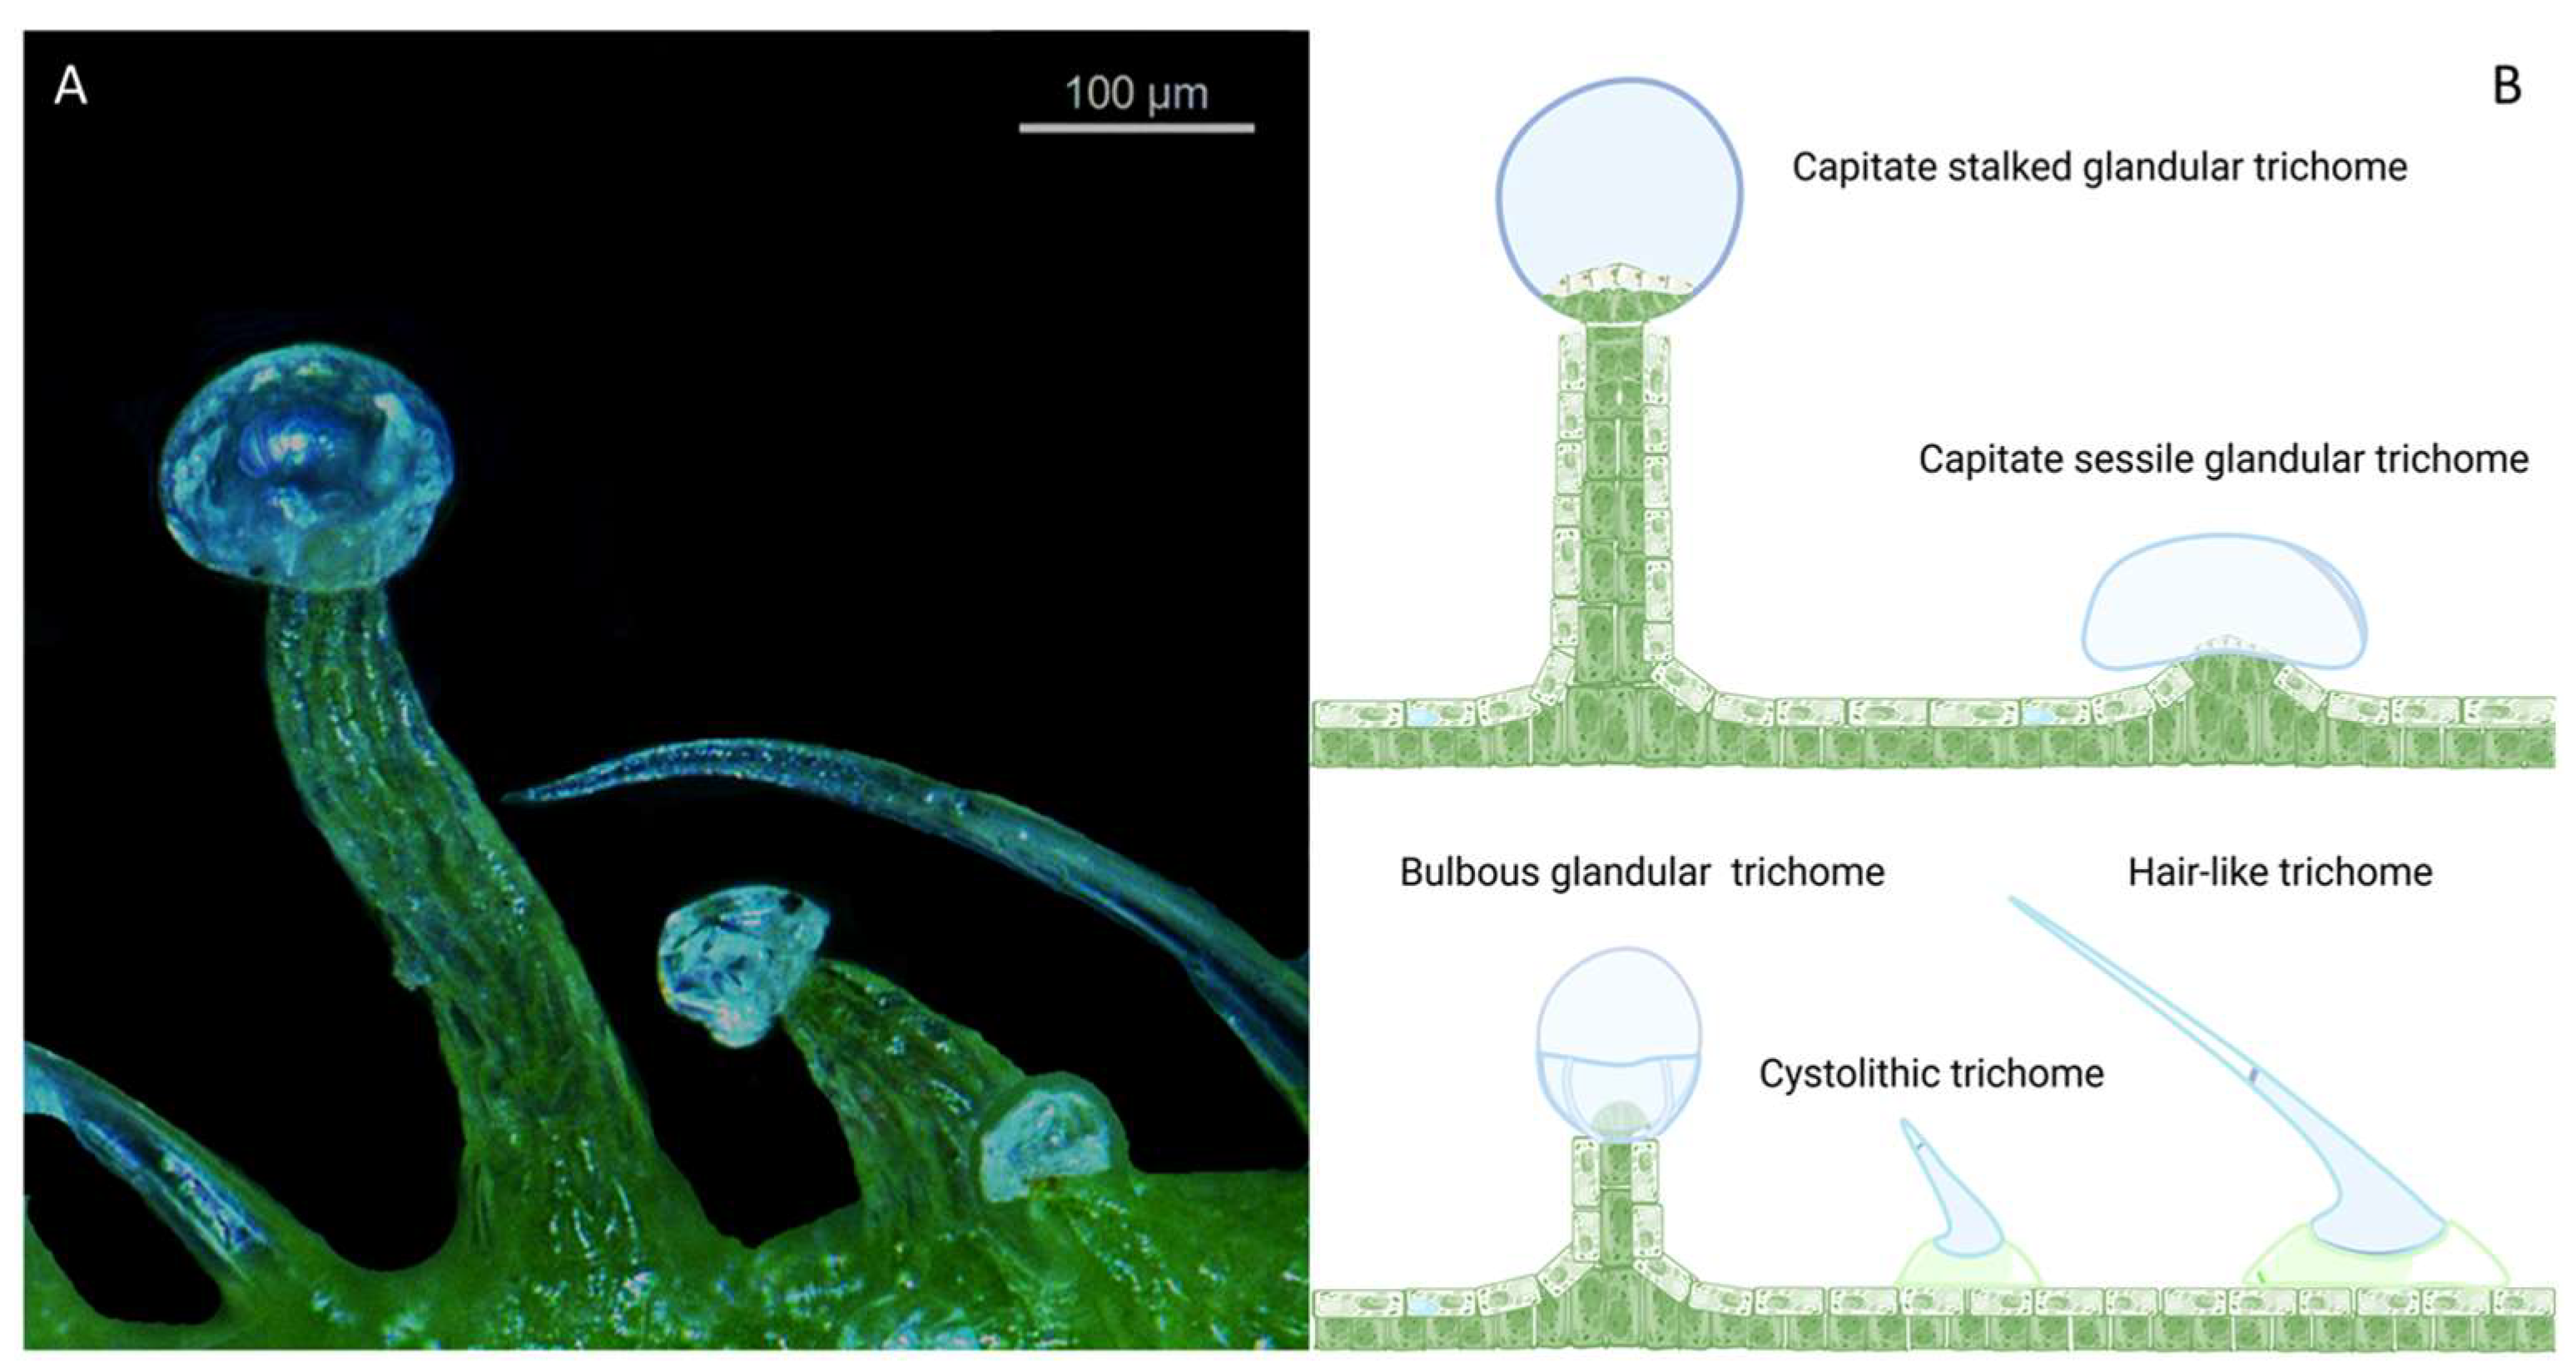
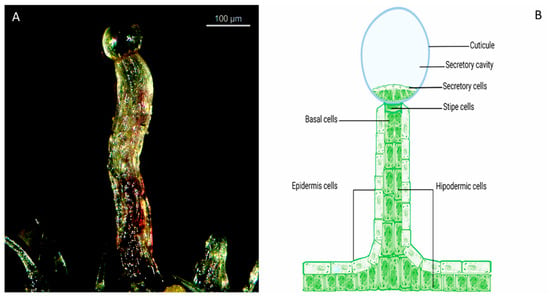
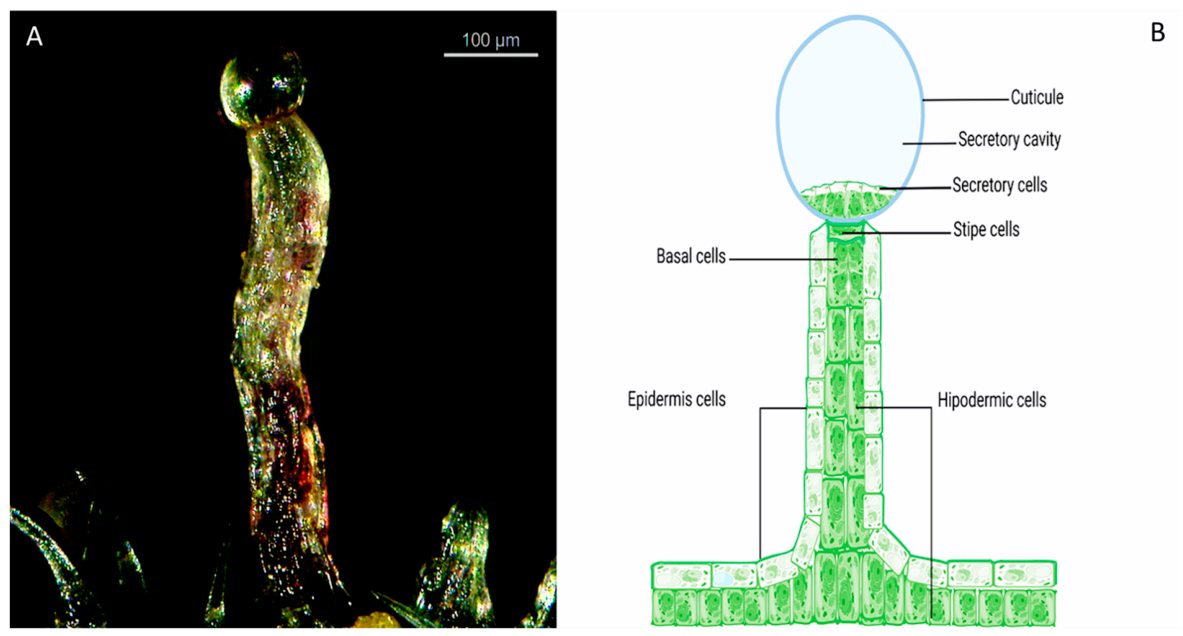
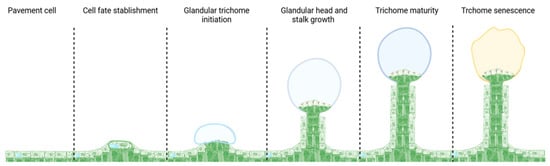
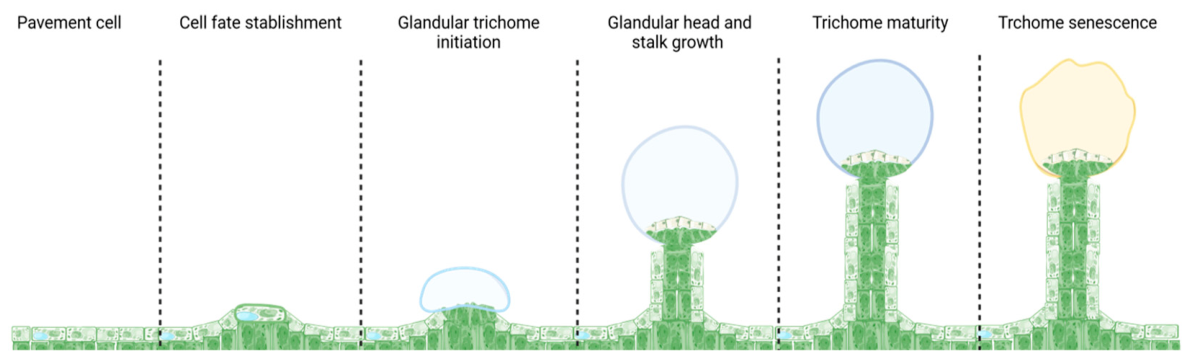
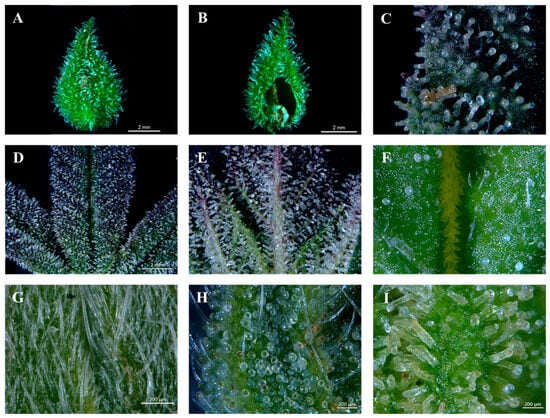
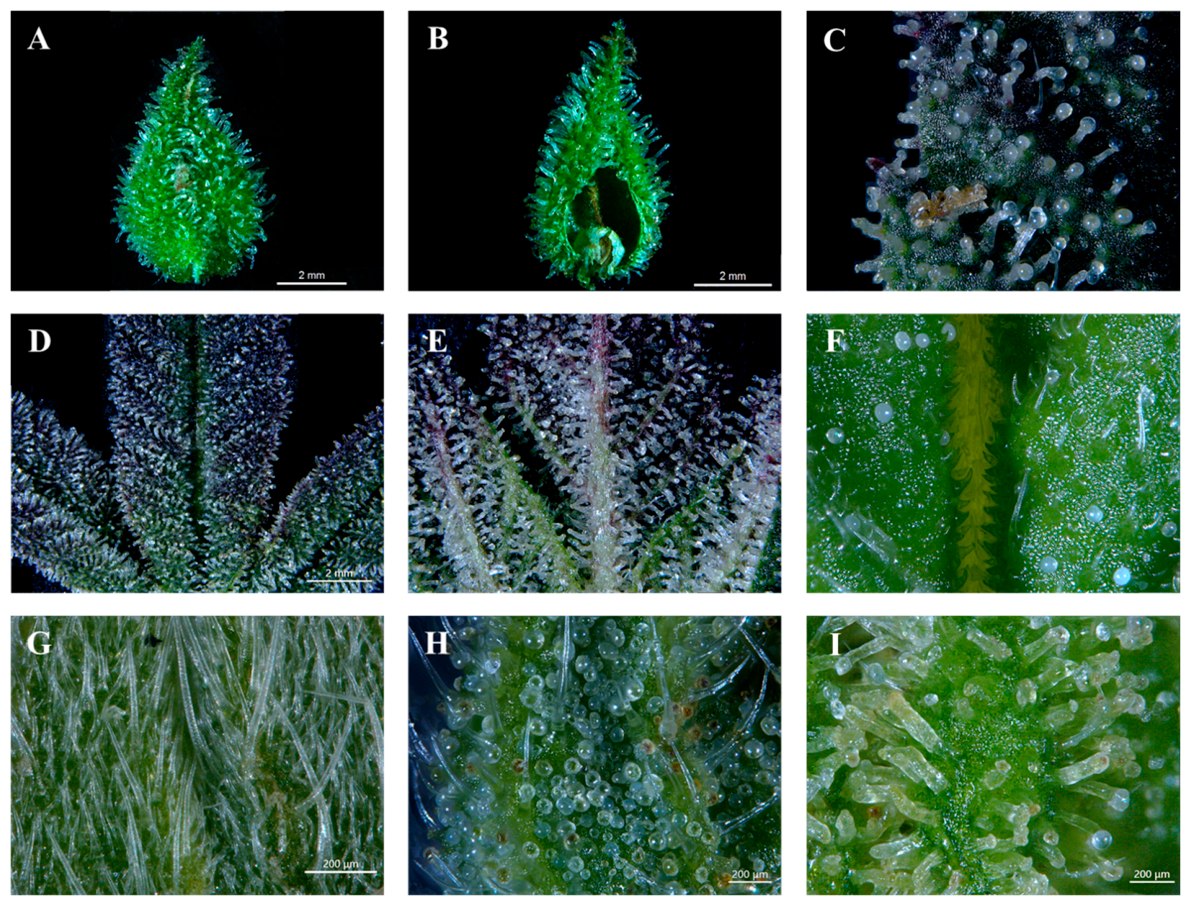
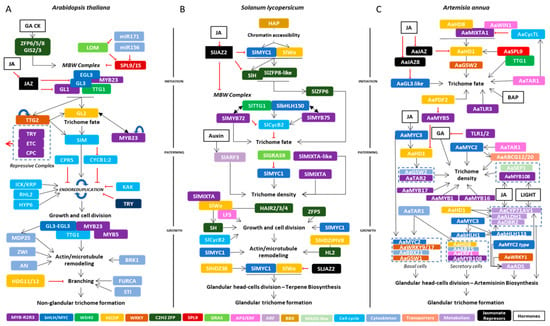
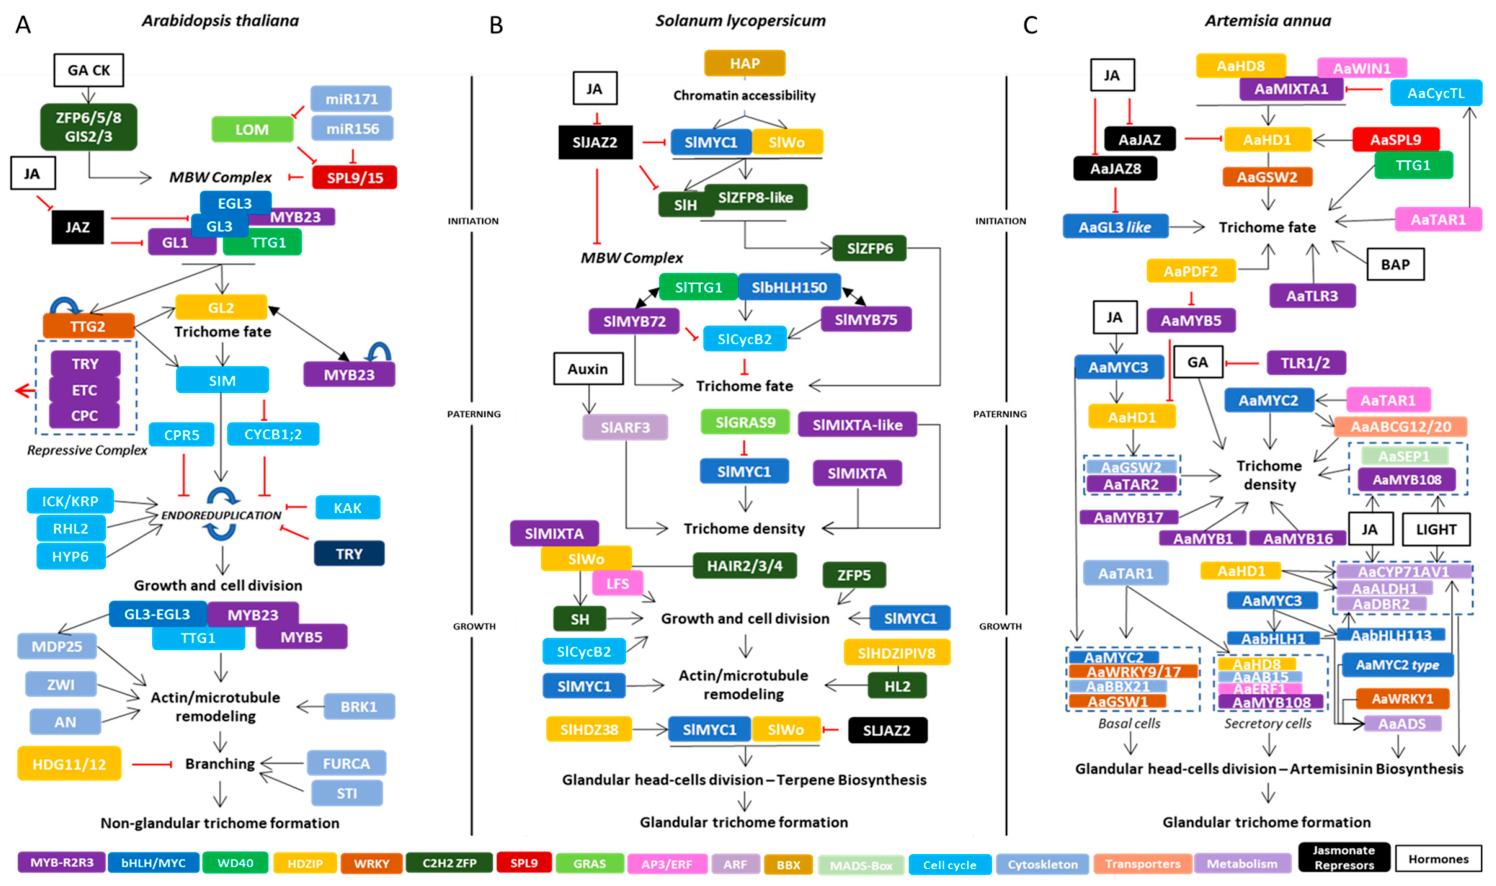
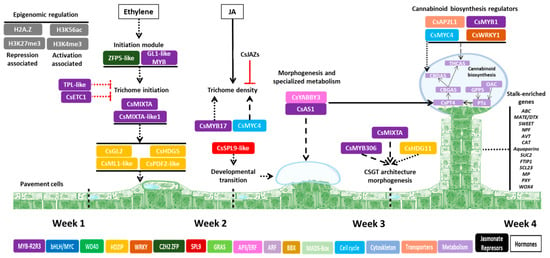
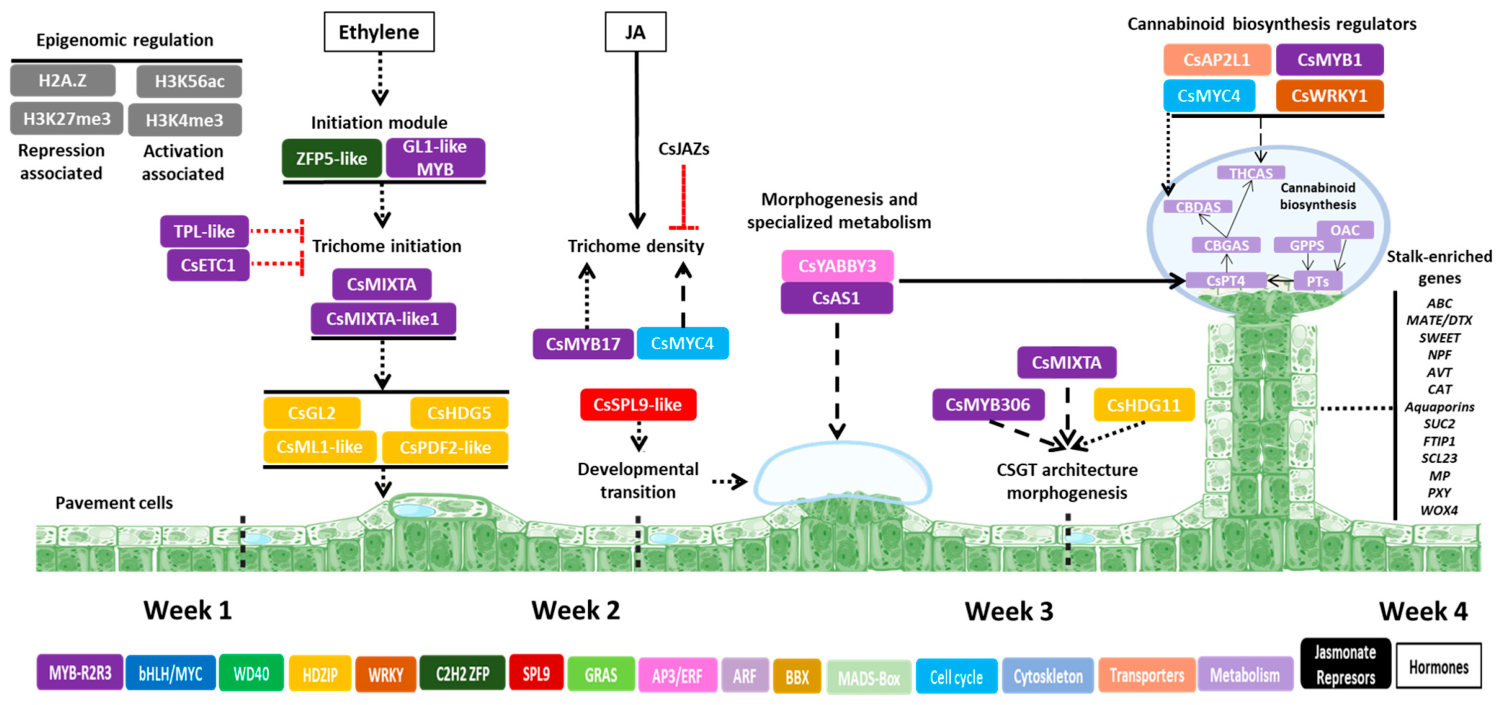

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.