


Abstract
Grassland degradation is a global ecological crisis that profoundly alters aboveground vegetation and soil properties, yet its impacts on soil microbial co-occurrence networks remain poorly understood. Here, we investigated soil bacterial and fungal communities along a well-defined five-stage degradation gradient spanning from non-degraded Leymus chinensis grassland to extremely degraded bare saline patches in the Songnen meadow steppe of northeastern China, using Illumina MiSeq sequencing and co-occurrence network analysis. Our results revealed that bacterial α-diversity exhibited a unimodal (hump-shaped) response peaking at the moderately degraded MD stage, whereas fungal diversity declined monotonically along the gradient, indicating greater sensitivity of fungi to degradation stress. Both bacterial and fungal community compositions shifted directionally with degradation, driven primarily by soil alkalization (pH) and electrical conductivity (EC). Network complexity followed a unimodal pattern for both kingdoms, maximizing at MD and collapsing at SD, suggesting a critical ecological threshold between moderate and severe degradation, while the increased proportion of positive correlations under severe degradation implied enhanced microbial cooperation in response to environmental stress. Structural equation models further revealed distinct regulatory pathways: bacterial networks were governed by both direct environmental filtering and indirect diversity-mediated effects, whereas fungal networks responded more strongly to direct pH/EC constraints and compositional shifts. Our findings demonstrate that microbial networks exhibit nonlinear threshold responses to grassland degradation, with fungi serving as more sensitive bioindicators than bacteria, and highlight the importance of integrating network-level properties into degradation monitoring and restoration frameworks.
1. Introduction
Grassland is one of the most widely distributed terrestrial ecosystems, covering approximately 40% of the Earth’s land surface, and plays an irreplaceable role in global nutrient cycling, biodiversity conservation, soil stabilization, and livestock production [1,2,3]. However, due to intensive anthropogenic activities—including overgrazing, agricultural intensification, and land-use change—coupled with climate variability, grassland degradation has become a global ecological challenge. According to the United Nations Convention to Combat Desertification (UNCCD), approximately 49% of global grasslands have experienced degradation to varying degrees, threatening ecosystem productivity, biodiversity, and ecological stability [4]. In China, an estimated 90% of grasslands have been degraded to varying degrees, posing serious threats to ecosystem productivity, stability, and regional sustainable development [5,6,7]. Grassland degradation is essentially a process of retrogressive succession, characterized by declining vegetation cover, aboveground biomass reduction, shifts in plant community composition from climax species (e.g., Leymus chinensis) to salt-tolerant pioneer species (e.g., Artemisia anethifolia, Suaeda spp.), and ultimately the formation of bare saline patches [8]. This continuous degradation gradient provides an ideal natural experimental platform for investigating the response of belowground ecological processes to ecosystem deterioration.
Soil microorganisms, comprising complex assemblages of bacteria, fungi, archaea, and viruses, are central to the functioning and resilience of grassland ecosystems [9]. They drive critical biogeochemical processes including organic matter decomposition, nitrogen fixation, phosphorus mobilization, and soil aggregate formation [10]. For instance, arbuscular mycorrhizal fungi (AMF) form extensive hyphal networks that enhance plant nutrient acquisition and drought tolerance, while nitrogen-fixing bacteria such as Rhizobium and Bradyrhizobium contribute substantially to the nitrogen economy of grasslands [11,12]. Given their sensitivity to environmental change, soil microbial communities often serve as early indicators of ecosystem stress and degradation [13,14]. Degraded grasslands are frequently characterized by reduced microbial biomass and diversity, breakdown of mutualistic interactions, and dominance of opportunistic or pathogenic taxa, leading to diminished soil quality and impaired recovery potential [15,16].
In recent years, there has been a paradigm shift in microbial ecology from merely describing community composition to understanding interspecific interactions and network dynamics [17]. Co-occurrence network analysis provides a powerful framework to infer potential ecological interactions (e.g., mutualism, competition, niche overlap) among microbial taxa and to characterize community-level topological properties such as complexity, connectivity, modularity, and stability [18,19]. These network attributes are increasingly recognized as critical determinants of ecosystem resistance and resilience to environmental perturbations [20,21]. For instance, complex networks with higher connectivity and redundancy are generally more resistant to species loss and environmental disturbances [22,23]. Conversely, network simplification—manifested as reduced nodes, links, and average degree—may indicate functional vulnerability and loss of ecosystem buffering capacity [24].
Despite growing interest, our understanding of how microbial co-occurrence networks respond along complete grassland degradation gradients remains fragmented and sometimes contradictory. Some studies report that degradation reduces microbial diversity and network complexity [25], while others reveal that degraded grasslands harbor more tightly connected networks as microbes strengthen cooperation to cope with environmental stress [9,15,26]. For example, research on the Qinghai–Tibet Plateau found that alpine grassland degradation increased fungal network complexity while decreasing bacterial and protistan network complexity, suggesting differential responses among microbial kingdoms [27]. Furthermore, studies in the Songnen Plain—a region characterized by low precipitation, high evaporation, saline parent material, and overgrazing—have shown that soil salinization and alkalization are primary filters shaping microbial community structure and function [28,29]. However, the relative importance of direct environmental filtering (e.g., pH, electrical conductivity) versus indirect vegetation-mediated pathways (e.g., reduced plant biomass and litter inputs) in driving network changes remains poorly resolved [30]. Moreover, whether bacteria and fungi exhibit consistent or divergent network responses across degradation stages has not been systematically examined, particularly in saline–alkaline meadow steppe ecosystems [31].
To address these knowledge gaps, we conducted a field study along a well-defined five-stage degradation gradient in the Songnen Grassland Ecosystem National Observation and Research Station, Northeast China. The gradient spans from non-degraded Leymus chinensis grassland (ND), through lightly degraded mixed forbs (LD), moderately degraded Artemisia anethifolia (MD), severely degraded Artemisia + Suaeda/Kochia (SD), to extremely degraded bare crust/vegetation patches (ED). This sequence represents a continuous retrogressive succession driven by soil salinization and alkalization, providing an ideal context for investigating gradual microbial responses.
Specifically, our study aimed to address the following questions: (1) How do bacterial and fungal community diversity, composition, and co-occurrence network topology change along the degradation gradient? (2) Do bacteria and fungi exhibit divergent network responses to degradation? (3) What are the key environmental drivers—direct soil physicochemical factors versus indirect vegetation-mediated pathways—that regulate microbial network changes? We hypothesized that (i) degradation would progressively simplify microbial networks, with the most drastic changes occurring between moderate and severe degradation stages; (ii) fungal networks would be more sensitive to degradation than bacterial networks due to their stronger dependence on vegetation inputs; and (iii) soil alkalization and salinization would serve as primary direct drivers, while vegetation biomass loss would exert indirect effects through reducing resource availability. By elucidating the patterns and drivers of microbial network changes along a complete degradation gradient, this study aims to provide a theoretical basis for developing microbial indicators of grassland degradation and informing restoration strategies.
2. Materials and Methods
2.1. Study Site Description
This study was conducted in August 2024 at the Jilin Songnen Grassland Ecosystem National Observation and Research Station, Northeast Normal University, Jilin Province, China (44°45′ N, 123°45′ E). The site is located in the low-lying area of the Songnen Plain, with relatively flat terrain at an elevation of 138–167 m above sea level. The region has a semi-arid continental monsoon climate, characterized by cold, dry winters and warm, rainy summers. Mean annual temperature ranges from 4.6 to 6.4 °C, and mean annual precipitation varies between 280 and 400 mm, with most rainfall occurring during the growing season (June to August). Annual evaporation (1200–1600 mm) is three to four times higher than precipitation. Soils are classified as castaneozem, light chernozem, and meadow chernozem, with pH values ranging from 7.0 to 10.5. Low precipitation, high surface evaporation, saline parent material, and overgrazing are the primary drivers of soil salinization and grassland degradation in this region. The dominant vegetation is the perennial rhizomatous grass Leymus chinensis, a common species in the eastern Eurasian steppes. Other common species include Phragmites australis, Calamagrostis epigejos, Artemisia scoparia, and Messerschmidia sibirica.
2.2. Experimental Design and Sampling
Five degradation stages were selected based on vegetation community composition and soil properties: non-degraded Leymus chinensis grassland (ND), lightly degraded mixed-forb community (LD), moderately degraded Artemisia anethifolia community (MD), severely degraded Artemisia + Suaeda/Kochia community (SD), and extremely degraded bare crust/vegetation patches (ED). At each degradation stage, six plots (25 m × 25 m) were established as independent replicates.
Vegetation sampling was conducted in mid-August. Within each plot, four parallel transects (25 m) were set at 5 m intervals, and 50 cm × 50 cm quadrats were placed along each transect at 5 m intervals. Aboveground living plants from 16 quadrats per plot were harvested, oven-dried at 65 °C for 48 h, and weighed to determine biomass. Plant species richness was recorded in each quadrat. Litter biomass was collected separately and weighed. Plant carbon and nitrogen concentrations were measured using a Vario MICRO cube Elemental Analyzer (Elementar GmbH, Hanau, Germany).
Soil samples were collected from the top 0–10 cm layer using a soil auger (5 cm diameter). Five soil cores were randomly collected from each subplot, mixed thoroughly, and homogenized to form one composite sample. After removing roots and plant residues, each sample was sieved through a 2 mm mesh and divided into three portions: one stored at −80 °C for DNA extraction, one kept at 4 °C for soil physicochemical analyses, and one air-dried at room temperature for total carbon and nitrogen determination. Soil pH and electrical conductivity (EC) were measured in a 1:5 (soil:water) suspension. Soil organic carbon (SOC) was determined using the K2Cr2O7 oxidation method. Soil NO3−-N and available phosphorus (AP) were measured using a continuous flow analyzer (Futura, Alliance, Frépillon, France) following standard protocols.
2.3. DNA Extraction, PCR Amplification, and Sequencing
Microbial DNA was extracted from 0.4 g of frozen soil using the MOBIO PowerSoil DNA Extraction Kit (MoBio Laboratories, Carlsbad, CA USA) following the manufacturer’s instructions. DNA quality was verified by 1% agarose gel electrophoresis. Bacterial 16S rRNA genes were amplified using primer pairs 338F (5′-ACTCCTACGGGAGGCAGCAG-3′) and 806R (5′-GGACTACHVGGGTWTCT AAT-3′), targeting the V3–V4 region. Fungal ITS regions were amplified using primers ITS1 (5′-CTTGGTCATTTAGAGGAAGTAA-3′) and ITS2 (5′-GCTGCGTTCTTCATCGATGC-3′). PCR products were purified using the AxyPrep DNA Gel Extraction Kit (Axygen Biosciences, Union City, CA, USA), quantified with QuantiFluor™-ST (Promega, Madison, WI, USA), and sequenced on the Illumina MiSeq platform (Majorbio, Shanghai, China).
2.4. Bioinformatics and Network Analysis
Raw sequences were demultiplexed, quality-filtered using fastp (version 0.20.0), and merged using FLASH (version 1.2.7). Operational taxonomic units (OTUs) were clustered at 97% similarity using UPARSE (version 7.1), and chimeric sequences were removed. Taxonomic assignment was performed using the RDP Classifier against the SILVA database (version 119) for bacteria and the UNITE database (version 7.0) for fungi, with a confidence threshold of 70%. To account for sequencing depth variation, samples were rarefied to the minimum sequence number (25,586 for bacteria; 32,000 for fungi) prior to downstream analysis. Alpha diversity indices (Shannon, Simpson, observed richness, Chao1, ACE) were calculated using mothur. Beta diversity was assessed via non-metric multidimensional scaling (NMDS) based on Bray–Curtis distances. To verify that significant PERMANOVA results were not driven by differences in within-group dispersion, homogeneity of multivariate dispersions was assessed using the betadisper function based on Bray–Curtis dissimilarities, followed by permutation tests (999 permutations). Co-occurrence networks were constructed at the genus level based on Spearman’s rank correlations. Considering that amplicon sequencing data are compositional, methods specifically designed for compositional microbiome data, such as SparCC and SPIEC-EASI, have been developed to reduce potential biases caused by relative abundance constraints. However, the objective of this study was to compare the relative changes in microbial network structure and complexity among different grassland degradation stages rather than to infer absolute microbial interactions. Therefore, Spearman correlation-based networks were constructed following previous ecological network studies. A stringent correlation threshold (|ρ| > 0.6) combined with a significance threshold (p < 0.01) was applied to retain only strong and statistically significant associations, thereby reducing weak or potentially spurious correlations. The same criteria were consistently applied to all degradation stages to ensure comparability among networks. Networks were visualized using Gephi (version 0.9.2) with a Fruchterman–Reingold layout. Topological parameters (nodes, links, average degree, modularity, average path length, clustering coefficient) were calculated using the igraph package in R (version 4.5.2).
2.5. Statistical Analysis
One-way analysis of variance (ANOVA) followed by Tukey’s HSD post hoc test was used to compare vegetation characteristics, soil physicochemical properties, and microbial alpha diversity indices across the five degradation stages. Permutational multivariate analysis of variance (PERMANOVA, Adonis) with 999 permutations was performed to test for significant differences in microbial community structure (β-diversity) among stages, based on Bray–Curtis distance matrices. Non-metric multidimensional scaling (NMDS) was employed to visualize the dissimilarities in bacterial and fungal community composition across degradation gradients.
To disentangle the direct and indirect effects of environmental drivers (soil pH, EC, vegetation biomass, microbial α-diversity, and β-diversity) on microbial co-occurrence network properties (average degree as a proxy for network complexity), we constructed partial least squares structural equation models (PLS-SEM) using the plspm (version 0.6.0) package in R (version 4.5.2). Prior to model construction, all variables were standardized to achieve a mean of zero and unit variance. The model fit was evaluated using the goodness-of-fit index (GOF), standardized root mean square residual (SRMR), and the coefficient of determination (R2) for endogenous variables. Path coefficients and their significance were estimated using bootstrap resampling with 1000 iterations. The total, direct, and indirect effects were calculated to partition the relative importance of each pathway. Model adequacy was confirmed by GOF > 0.6 and SRMR < 0.08. All statistical analyses were performed using R software (version 4.5.2) with packages vegan (version 2.7-3), igraph (version 2.2.1), psych (version 2.6.1), ggplot2 (version 4.0.2), and plspm (version 0.6.0). Statistical significance was set at p < 0.05 unless otherwise specified. All data are presented as mean ± standard deviation (SD).
3. Results
3.1. Vegetation and Soil Properties Along the Degradation Gradient
Plant community structure deteriorated progressively along the ND → LD → MD → SD → ED gradient (Table 1). Species richness declined from 5.67 ± 2.07 in ND to near-zero in ED (F = 32.10, p < 0.001), while total biomass decreased from 458.01 ± 98.72 g m−2 in ND to 364.35 ± 96.76 g m−2 in MD, collapsed completely in SD, and partially recovered in ED (247.34 ± 75.14 g m−2) due to colonization by salt-tolerant pioneer species. Litter biomass exhibited the most dramatic reduction, decreasing by approximately 84% from LD to MD and approaching zero in SD and ED (F = 105.87, p < 0.001), indicating near-complete cessation of organic matter return to soil under advanced degradation.
Table 1.
Soil physicochemical properties along the grassland degradation gradient.
Soil properties underwent systematic modification along the gradient (Table 1). Soil pH shifted from mildly alkaline in ND (8.38 ± 0.15) and LD (8.05 ± 0.06) to extremely alkaline in MD–ED (9.70–10.01; F = 212.50, p < 0.001), accompanied by progressive accumulation of soluble salts and exchangeable cations (Na+ increased from 0.008 to 1.880 cmol kg−1; F = 124.60, p < 0.001). Soil organic carbon decreased by 37.7% from ND to ED (F = 89.30, p < 0.001), while NO3−-N and available P accumulated exceptionally in ED (38.20 and 28.91 mg kg−1, respectively), suggesting nutrient cycling decoupling under severe degradation.
3.2. Shifts in Soil Microbial Diversity Along the Degradation Gradient
Bacterial α-diversity showed a unimodal pattern along the degradation gradient, with the highest diversity observed at the moderately degraded stage (MD) and a sharp decline under severe degradation (SD) (Table 2). In contrast, fungal α-diversity was relatively stable during early and intermediate degradation but decreased under advanced degradation stages. These contrasting patterns indicate that bacteria were more sensitive to environmental deterioration, whereas fungi maintained greater resistance during early degradation.
Table 2.
Bacterial and fungal α- and β-diversity across degradation stages (mean ± SD).
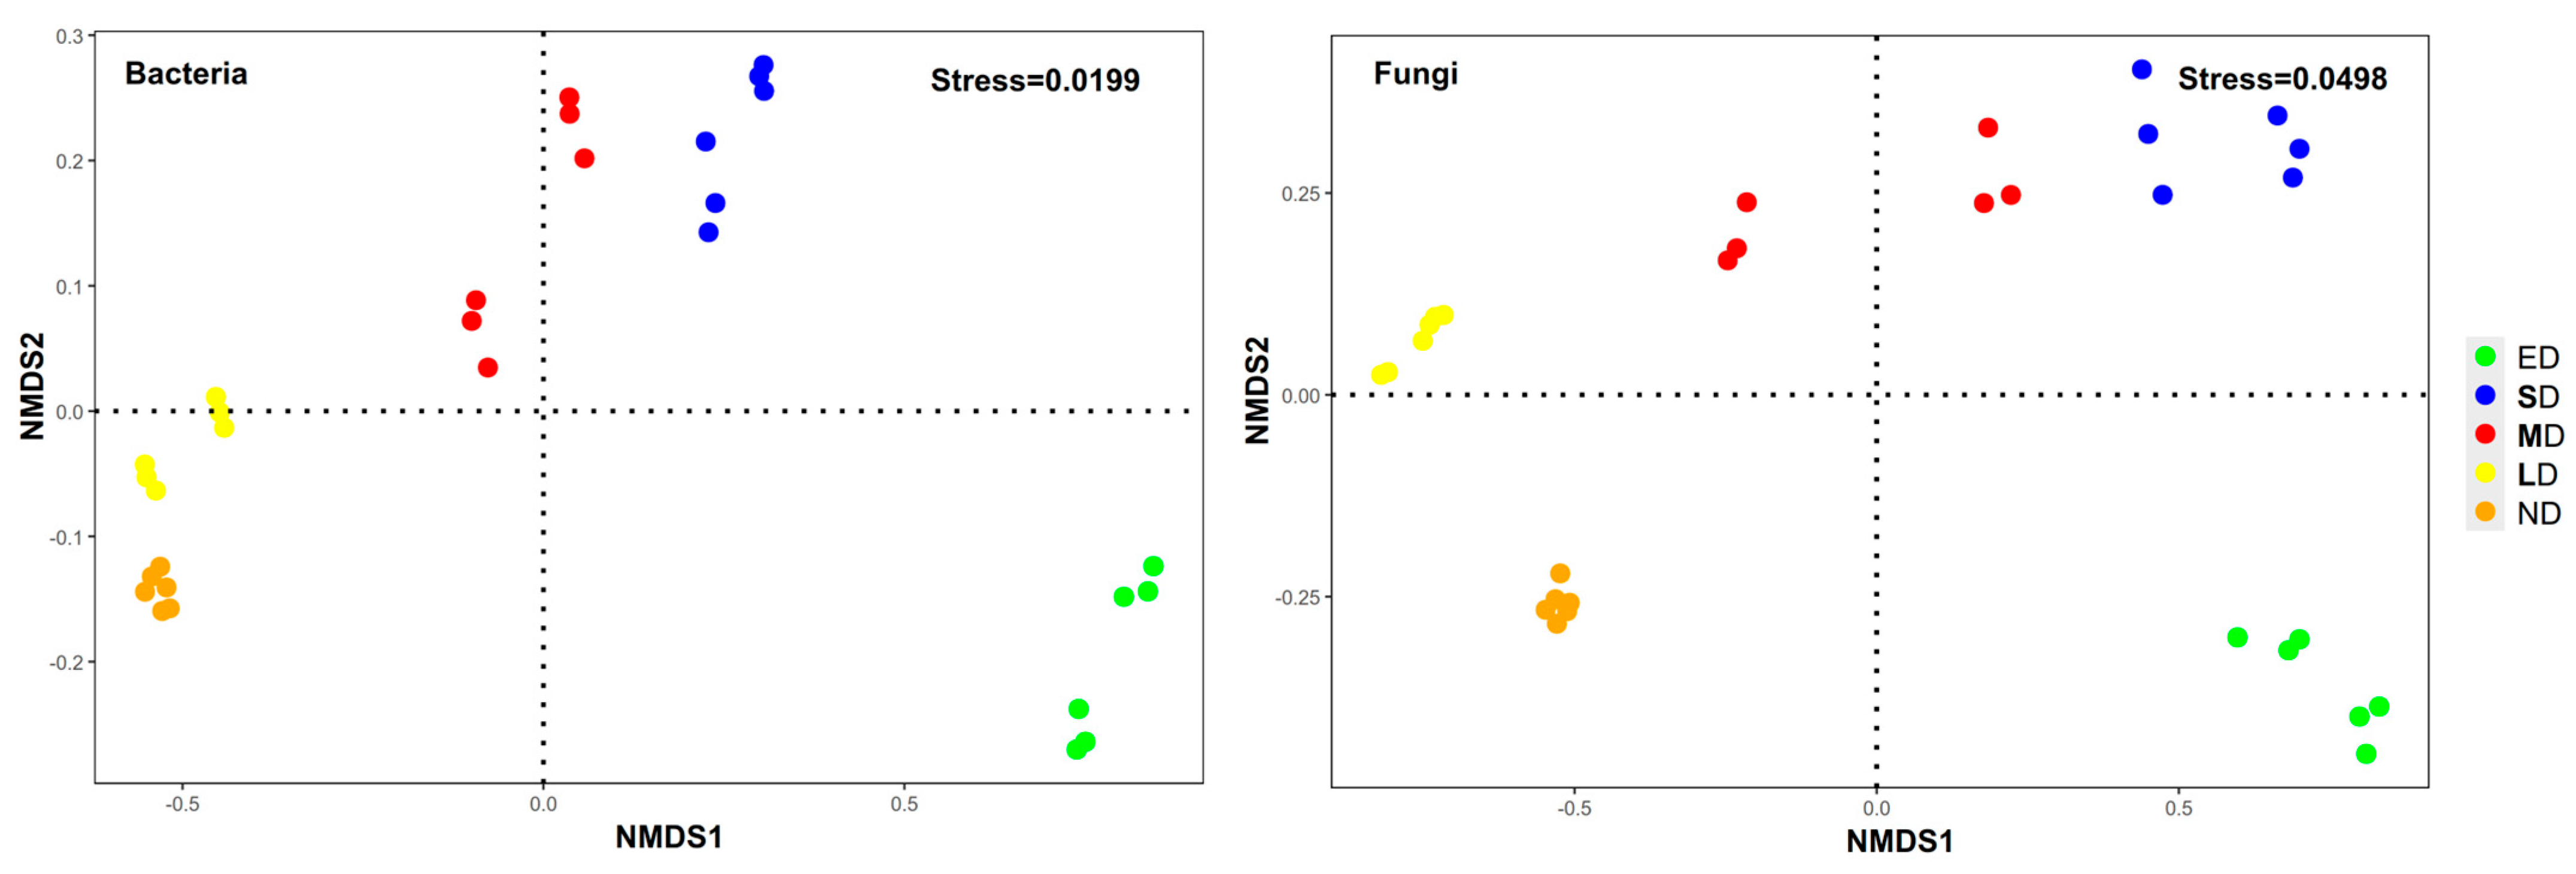
Both bacterial and fungal communities exhibited significant compositional shifts along the degradation gradient. NMDS ordination based on Bray–Curtis dissimilarity showed clear separation among degradation stages, and PERMANOVA confirmed that degradation stage explained 61.2% and 58.3% of bacterial and fungal community variation, respectively (p < 0.001)(Figure 1). PERMDISP analysis showed no significant differences in bacterial community dispersion among degradation stages (F = 1.9664, p = 0.128), indicating that bacterial community differentiation mainly reflected shifts in community centroids. In contrast, fungal communities exhibited significant differences in within-group dispersion (F = 22.839, p = 0.001), suggesting that fungal community restructuring involved both changes in community composition and increased variability among degradation stages.
Figure 1.
NMDS ordination of soil bacterial and fungal communities along the grassland degradation gradient based on Bray–Curtis dissimilarity. ND, non-degraded Leymus chinensis grassland; LD, lightly degraded mixed-forb community; MD, moderately degraded Artemisia anethifolia community; SD, severely degraded Artemisia + Suaeda/Kochia community; ED, extremely degraded bare crust/vegetation-free patches.
3.3. Degradation-Induced Shifts in Microbial Co-Occurrence Network Topology
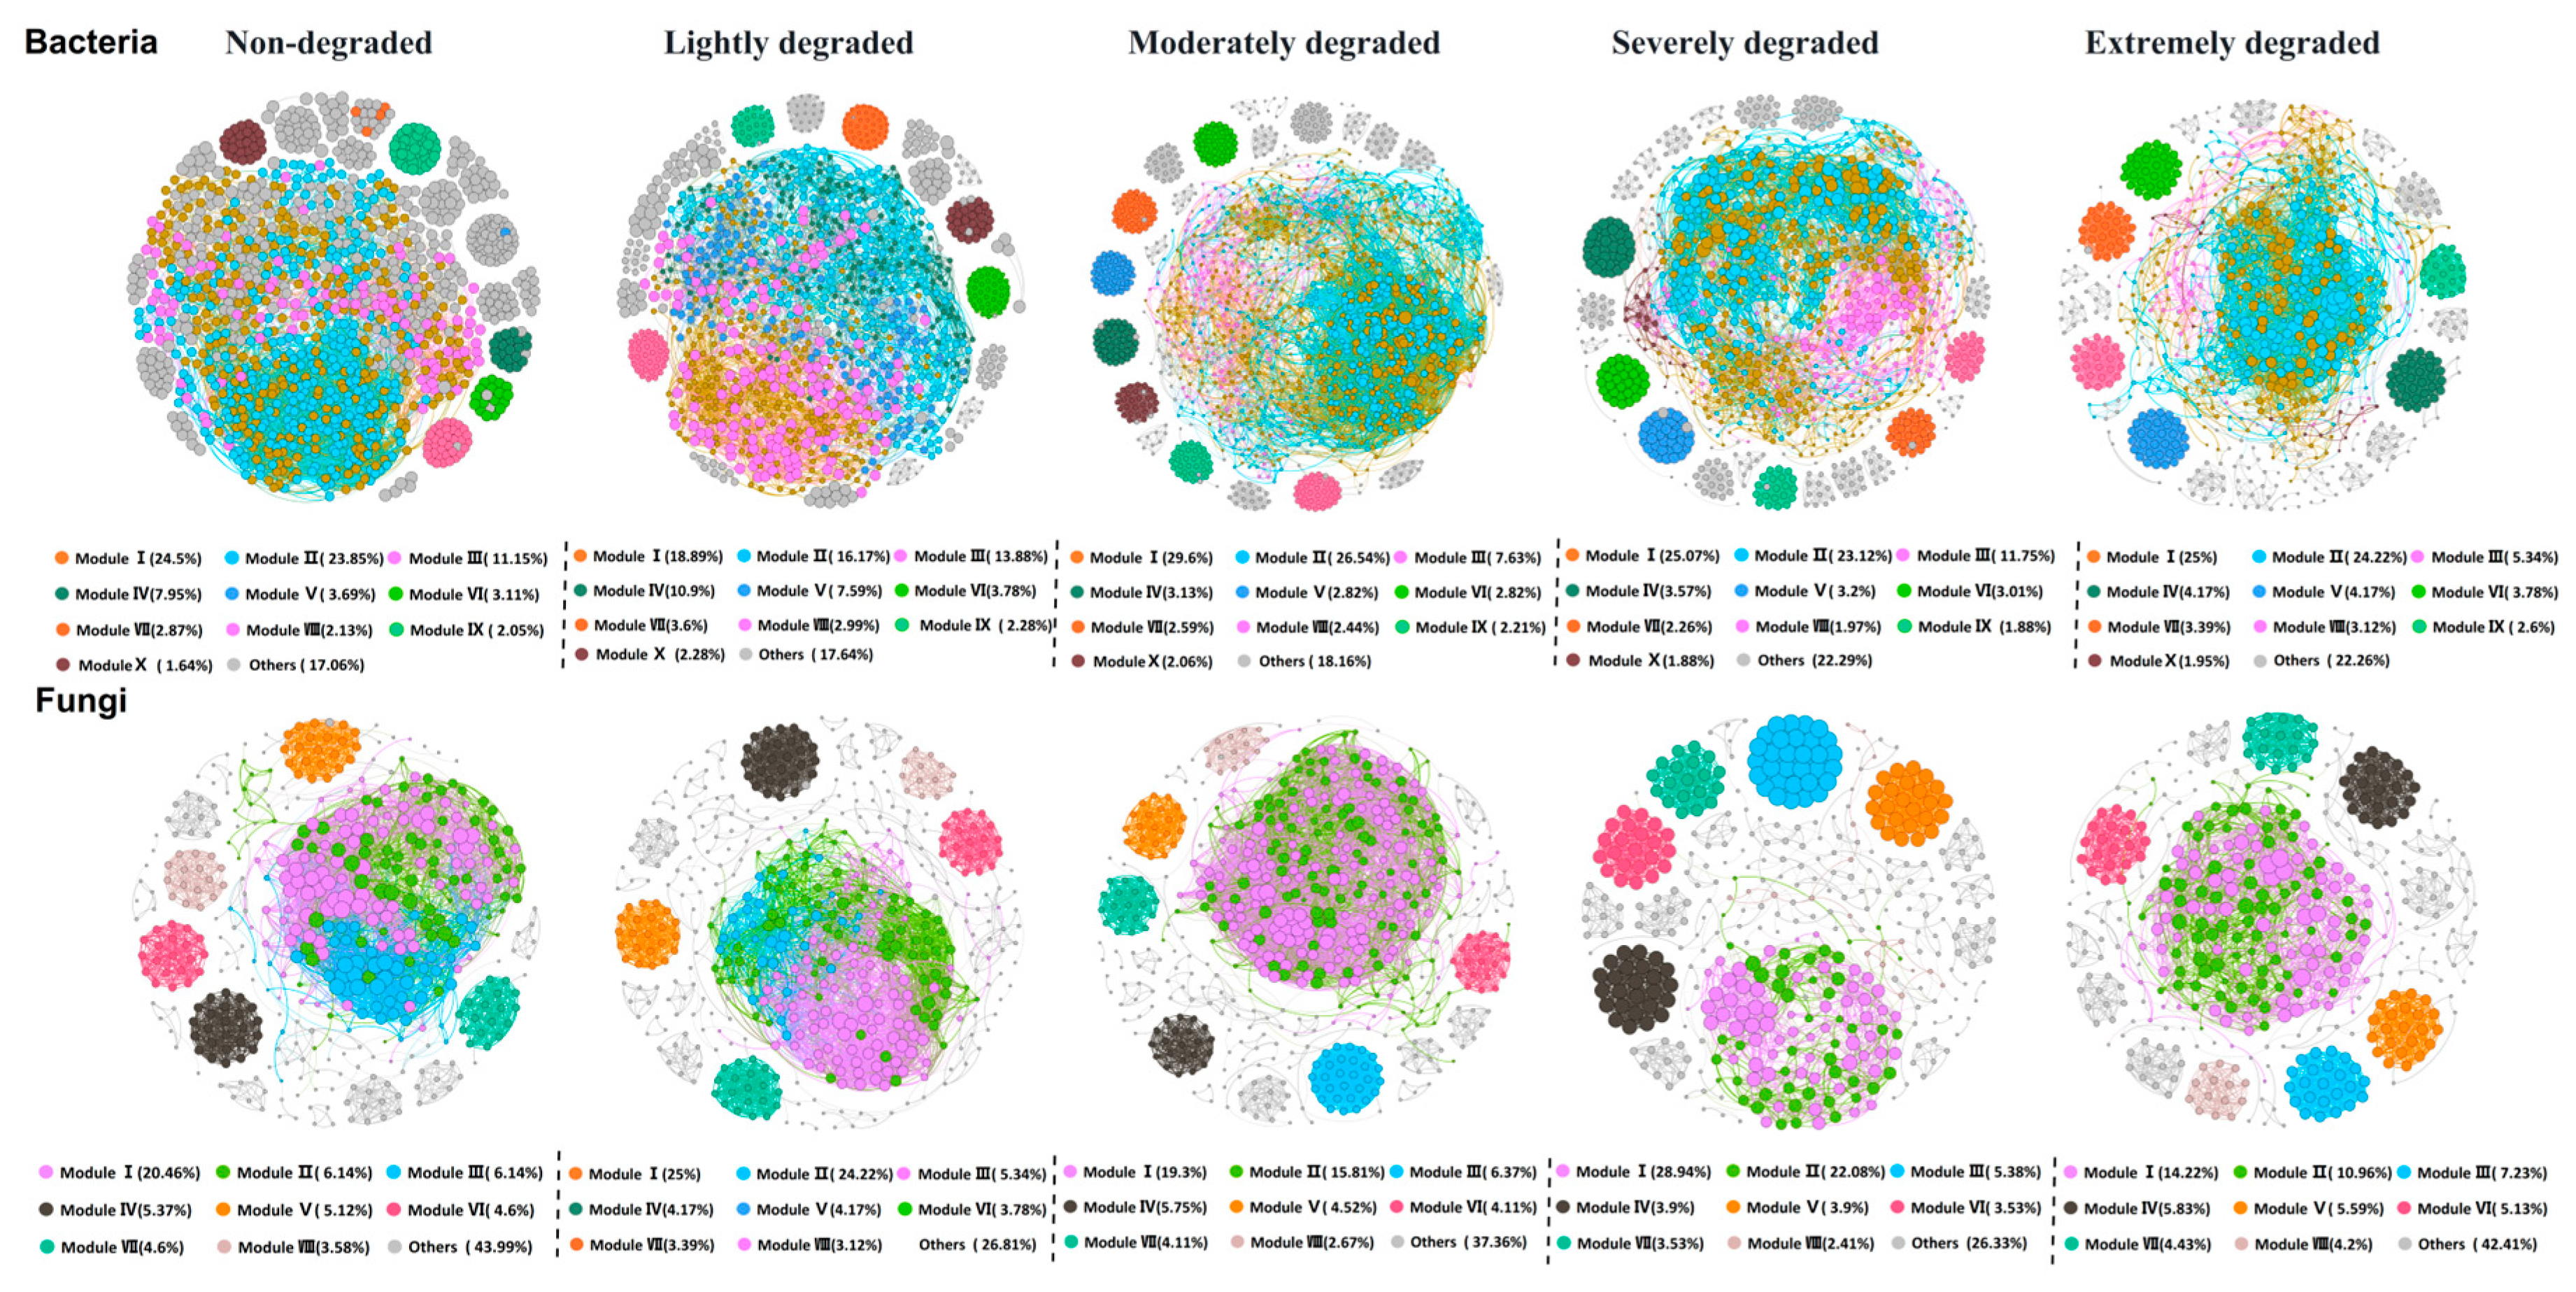
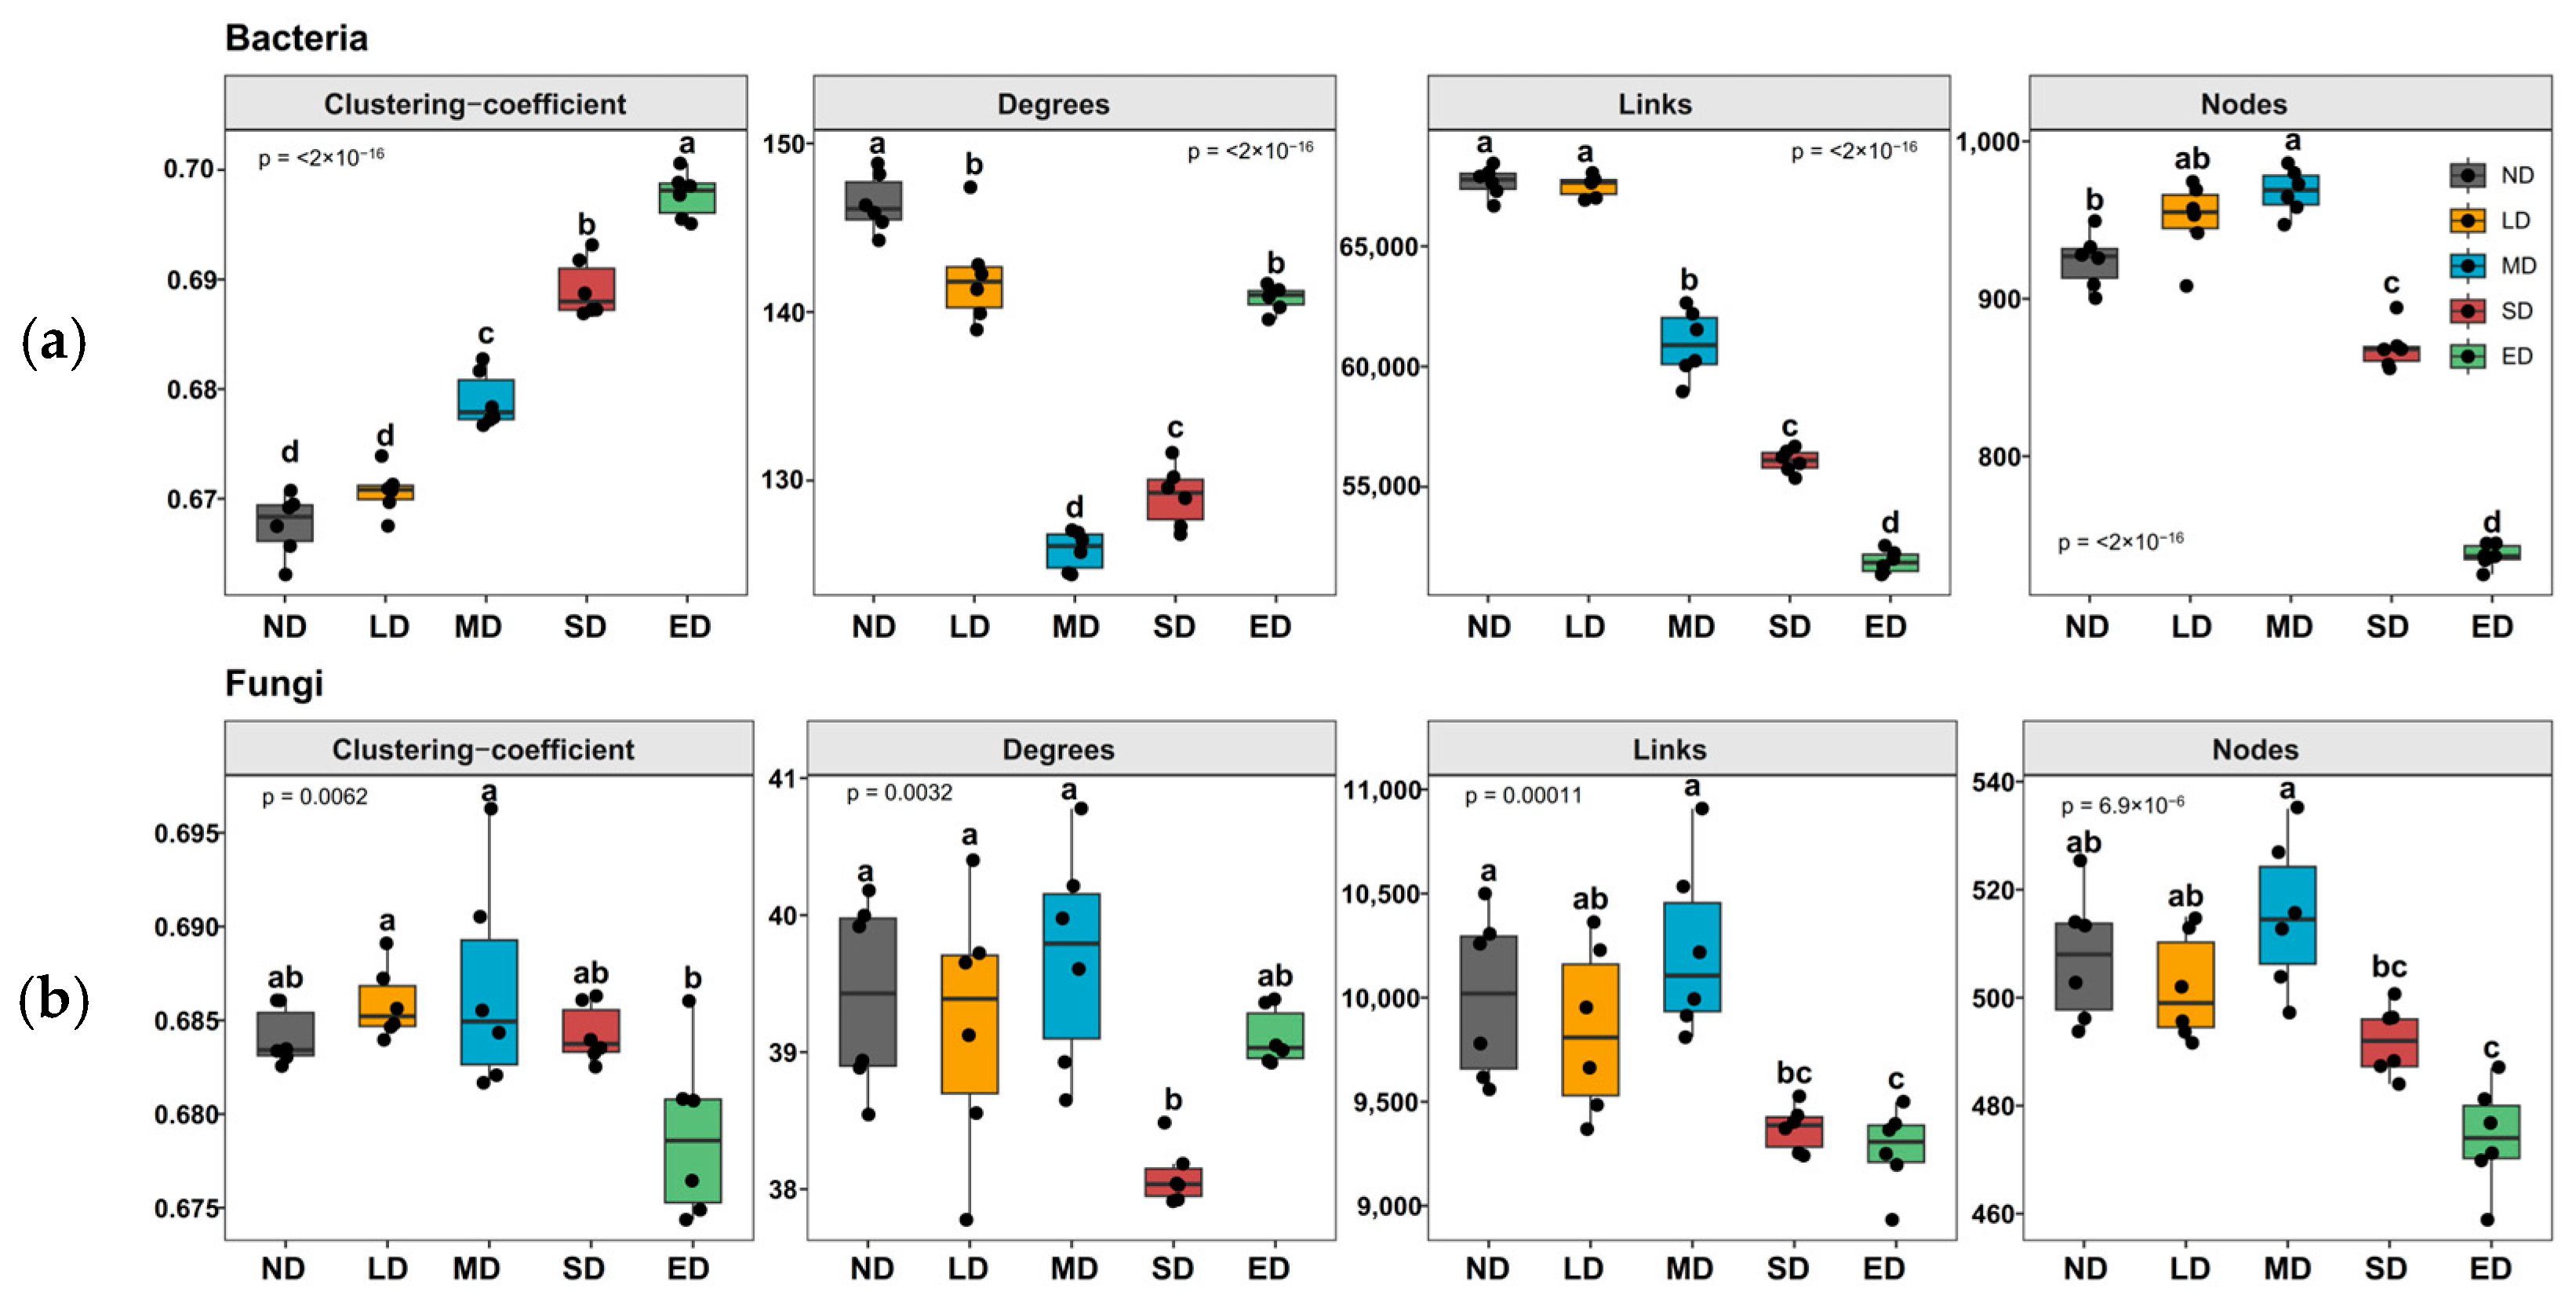
Bacterial and fungal co-occurrence networks exhibited pronounced changes along the degradation gradient (Figure 2 and Figure 3). For bacterial networks, nodes and links followed a unimodal pattern, increasing from ND (1220 nodes, 12,860 links) to MD (1311 nodes, 16,989 links), then declining sharply in SD (768 nodes, 6993 links). Average degree peaked at MD (25.918) and was the lowest in SD (18.211). Network modularity showed a decreasing trend from ND (0.834) to MD (0.724), followed by a slight increase at SD (0.782) and ED (0.745). Meanwhile, the clustering coefficient increased from LD (0.655) to ED (0.703), suggesting enhanced local connectivity and tighter microbial associations under advanced degradation stages.
Figure 2.
Co-occurrence networks of bacterial and fungal communities across five degradation stages. Nodes represent microbial genera, with node size proportional to degree. Non-degraded, Leymus chinensis grassland; lightly degraded, mixed forbs; moderately degraded, Artemisia anethifolia; severely degraded, Artemisia + Suaeda/Kochia; extremely degraded, bare crust.
Figure 3.
Co−occurrence networks of soil bacterial (a) and fungal (b) communities across five degradation stage. ND, Leymus chinensis grassland; LD, mixed forbs (lightly degraded); MD, Artemisia anethifolia; SD, Artemisia + Suaeda/Kochia (severely degraded); ED, bare crust (extremely degraded). Significant differences (p < 0.05) between different straw incorporation treatments are marked with different letters.
Fungal networks showed similar trends but with lower overall complexity. Links increased from LD (4340) to MD (6584) and then decreased to 2800 in SD, while average degree followed the same pattern (LD: 17.823 → MD: 24.430 → SD: 13.054). Average path length decreased from LD (5.179) to MD (3.620), then increased sharply in SD (5.764), indicating network fragmentation under extreme degradation. Notably, both bacterial and fungal networks exhibited a critical tipping point between MD and SD, with links decreasing by 59.5% and 57.5%, respectively, coinciding with the transition from moderate to severe degradation.
3.4. Turnover of Microbial Hub Taxa Along the Degradation Gradient
To identify the taxa contributing to microbial network restructuring, we further identified hub taxa based on node degree and betweenness centrality and analyzed their abundance changes along the degradation gradient (Tables S1 and S2). Bacterial hub taxa showed clear turnover across degradation stages. Early-stage networks were mainly associated with highly connected taxa such as Hirschia, Taibaiella, and Tumebacillus, whereas intermediate degradation promoted the emergence of Actinobacteriota-related hubs, including Phaselicystis and Glycomyces. Under severe degradation, bacterial networks were dominated by stress-adapted taxa, such as Acidobacteria-related groups and Desulfuribacillus. Fungal networks exhibited a similar replacement pattern, with early-stage hubs including Paraphaeosphaeria and Sarocladium being replaced by stress-tolerant taxa such as Plenodomus, Colletotrichum, and Preussia at advanced degradation stages. Several hub taxa showed high connectivity despite relatively low abundance, indicating that their ecological importance was associated with network interactions rather than dominance. These results suggest that degradation-induced network simplification was accompanied by the loss of key microbial hubs and the recruitment of stress-adapted taxa.
3.5. Drivers of Microbial Co-Occurrence Network Changes
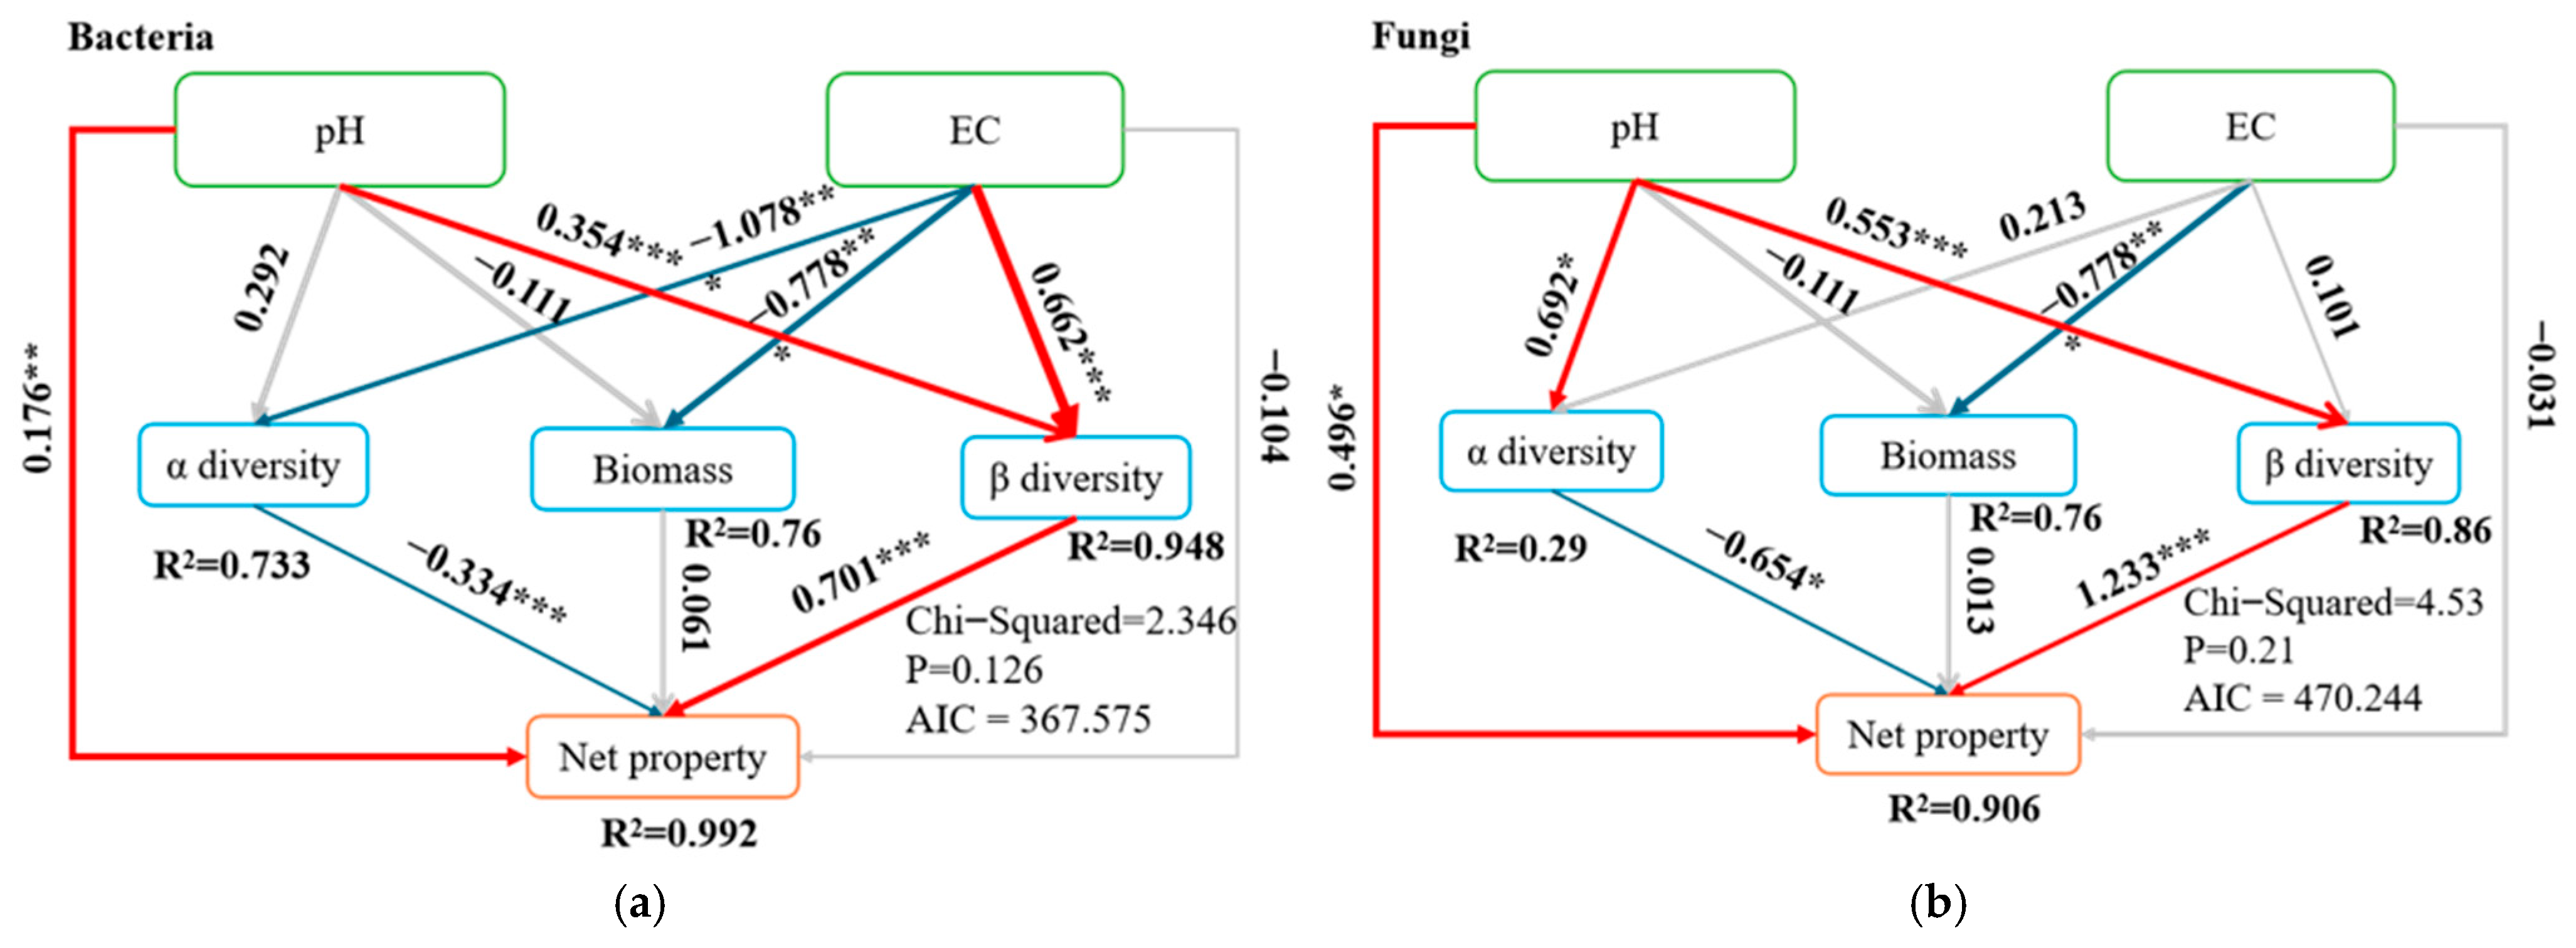
To identify the mechanisms driving microbial network restructuring during grassland degradation, SEM was constructed by integrating soil properties, vegetation biomass, microbial diversity, and the integrated network property index (Net property) (Figure 4). The models explained 99.2% and 90.6% of the variation in bacterial and fungal Net properties, respectively.
Figure 4.
Structural equation models (SEM) showing direct and indirect effects of environmental drivers on microbial network properties for bacteria (a) and fungi (b). Blue and red arrows indicate positive and negative relationships, respectively. Arrow width is proportional to standardized path coefficients (β). Numbers adjacent to arrows represent significant standardized path coefficients (* p < 0.05, ** p < 0.01, *** p < 0.001). Grey arrows indicate non-significant paths (p > 0.05). R2 values denote the proportion of variance explained for each endogenous variable. EC, electrical conductivity; α-diversity, Shannon diversity index; β-diversity, community compositional dissimilarity (NMDS1); Net property, the first principal component (PC1) derived from multiple co-occurrence network topological characteristics, including nodes, links, average degree, and clustering coefficient.
For bacterial communities, soil pH and EC were the primary environmental factors affecting community diversity and composition, indicating strong environmental filtering during degradation (Figure 4a). Bacterial Net property was more closely associated with changes in community composition (β-diversity) than α-diversity, suggesting that bacterial network restructuring was mainly driven by community turnover along the degradation gradient. For fungal communities, soil pH and EC also regulated network restructuring by influencing fungal diversity and community composition (Figure 4b). Similar to bacteria, β-diversity showed a stronger association with fungal Net property, highlighting the importance of community compositional shifts in fungal network assembly. Overall, SEM revealed that environmental filtering and microbial community turnover were key pathways regulating network changes, with compositional restructuring playing a central role in both bacterial and fungal networks.
4. Discussion
4.1. Soil Alkalization and Salt Accumulation as Primary Environmental Filters
Our results demonstrated that soil pH and electrical conductivity (EC) were the strongest environmental filters shaping microbial community composition and network structure along the degradation gradient. The dramatic increase in pH from 8.05 (LD) to 10.01 (SD) and the 235-fold increase in Na+ concentration from ND to SD represent the most pronounced edaphic responses to degradation. These findings align with studies in the Songnen alkaline salt-degraded grassland, where EC, pH, and available phosphorus (AP) were identified as the main drivers of soil bacterial community composition, while EC, pH, and soil organic carbon (SOC) primarily drove fungal community composition [28]. The extreme alkaline conditions (pH > 9.5) in MD, SD, and ED stages likely impose strong physiological constraints on microbial taxa, as high pH disrupts cellular homeostasis and enzyme activity.
The systematic shifts in the relative abundance of Actinobacteria, Firmicutes, Gemmatimonadetes, and Deinococcus–Thermus along the degradation gradient, together with the decline in Acidobacteria and Nitrospirae, suggest that salinity-related environmental filtering may influence bacterial community assembly. Studies in saline environments have identified Actinobacteria and Deinococcus–Thermus as halotolerant phyla that are frequently favored under salt-stressed conditions [32,33]. Deinococcus–Thermus, which showed a marked increase in relative abundance under severe degradation, is a phylum of extremophiles with exceptional resistance to radiation, desiccation, and oxidative stress, making it a potential indicator of severe degradation. Previous research on crude oil-contaminated saline soils has also identified Actinobacteria, Firmicutes, and Deinococcus–Thermus as dominant bacterial groups associated with environments experiencing salinization and contamination stresses [34]. Conversely, Acidobacteria, typically oligotrophic and adapted to acidic or neutral pH, declined sharply under alkaline conditions, consistent with their documented sensitivity to high pH. This compositional shift from copiotrophic to stress-tolerant strategists mirrors the “environmental filtering” paradigm, wherein abiotic conditions selectively eliminate poorly adapted taxa.
4.2. Divergent Diversity Responses: Bacterial Unimodality Versus Fungal Monotonic Decline
A striking finding of this study was the contrasting alpha diversity patterns between bacteria and fungi along the degradation gradient. Bacterial Shannon diversity exhibited a hump-shaped (unimodal) response, peaking at the moderately degraded MD stage, whereas fungal Shannon diversity decreased monotonically along the gradient. This divergence underscores fundamental differences in the ecological strategies and environmental sensitivities of these two microbial kingdoms.
The unimodal bacterial response was consistent with a disturbance-mediated diversity pattern predicted by the intermediate disturbance hypothesis (IDH), although this interpretation should be considered cautiously in microbial systems. Moderate degradation (MD stage) may generate increased environmental heterogeneity, altered resource availability, and transitional niches due to partial vegetation loss and increasing salinity stress, which could temporarily maintain higher bacterial diversity. However, the observed pattern may also reflect strong environmental filtering and shifts in microbial community assembly processes rather than disturbance effects alone [35,36]. However, as degradation intensifies beyond a critical threshold (the SD–ED transition), environmental stress exceeds the physiological tolerance of most taxa, leading to a sharp decline in diversity. Studies in the Songnen Plain have confirmed that saline–alkali degradation has a negative effect on microbial biodiversity, with different degradation gradients exhibiting different adaptability and tolerance species [28]. Therefore, the unimodal bacterial diversity pattern should not be interpreted as direct evidence supporting IDH, but rather as a response emerging from the combined effects of disturbance intensity, environmental filtering, and resource redistribution along the degradation gradient.
In stark contrast, fungal diversity declined consistently with increasing degradation, indicating that fungi are more sensitive to degradation than bacteria. This differential sensitivity can be attributed to several mechanisms. First, fungi, particularly mycorrhizal species, depend on living plant hosts for carbon substrates and are thus directly affected by vegetation degradation. Second, fungal hyphae are physically more vulnerable to soil structural disruption and desiccation than bacterial cells. Third, fungi generally lack the sophisticated osmoregulatory mechanisms found in many salt-tolerant bacteria. Studies on alpine cushion plant degradation have similarly found that fungal networks exhibited greater stability than bacterial networks, with bacterial networks being more vulnerable to environmental changes [37]. The progressive decline in plant diversity and biomass along the gradient, coupled with the loss of litter inputs, likely reduced the diversity of fungal substrates, as fungi are more dependent on plant-derived organic matter than bacteria. Thus, fungal communities may serve as more sensitive bioindicators of grassland degradation.
4.3. Network Responses to Degradation: Complexity Decline and Cooperative Shifts
Our co-occurrence network analysis revealed that both bacterial and fungal networks exhibited nonlinear responses along the degradation gradient, with most complexity-related properties (nodes, links, and average degree) peaking at MD and declining sharply under SD. The substantial reduction in links from MD to SD indicates a potential ecological threshold, where increasing environmental stress drives microbial network simplification. Similar nonlinear changes in microbial network organization have been observed during ecosystem degradation, suggesting that key degradation stages may trigger rapid network reorganization [37].
The decline in network complexity was accompanied by pronounced turnover of hub taxa. Resource-associated taxa that contributed to microbial interactions under less degraded conditions were gradually replaced by stress-adapted groups under advanced degradation. This indicates that network simplification was not merely caused by the loss of taxa, but also reflected functional restructuring of microbial interactions under environmental filtering.
Interestingly, although overall network complexity decreased, the proportion of positive correlations and clustering coefficient increased along the degradation gradient. This suggests that surviving microbial taxa may maintain stronger cooperative associations under severe stress, consistent with the stress gradient hypothesis (SGH), which predicts increased facilitative interactions under stressful environments [38,39]. In saline–alkaline ecosystems, enhanced microbial cooperation may involve metabolite exchange, substrate sharing, and biofilm formation. Recent studies have also reported increases in positive microbial associations under increasing saline–alkali stress, supporting the applicability of SGH at the microbial community level [40].
However, SGH responses may vary among ecosystems and stress gradients. Studies in saline ephemeral lakes showed that reduced competition did not necessarily correspond to increased facilitation, indicating that stress effects on microbial interactions are context-dependent [40,41]. Therefore, network complexity and interaction intensity should be considered as complementary but distinct properties, as microbial networks may simultaneously exhibit reduced connectivity and enhanced local cooperation under severe environmental stress.
4.4. Distinct Drivers of Bacterial and Fungal Networks: Direct Versus Indirect Pathways
Our SEM results revealed that microbial network restructuring during grassland degradation was jointly regulated by environmental filtering and community turnover. By integrating multiple network topological properties into a Net property index, we demonstrated that soil conditions and microbial community changes were key drivers of network variation.
For bacterial communities, soil pH and EC acted as important environmental filters shaping network organization. Increasing soil alkalinity significantly reduced bacterial α-diversity, while simultaneously promoting shifts in bacterial community composition, indicating that alkaline–saline stress selectively constrained bacterial taxa and altered community assembly. The positive association between β-diversity and bacterial Net property suggests that compositional turnover among degradation stages was closely linked with bacterial network restructuring. This pattern indicates that degradation did not simply reduce microbial interactions but reorganized bacterial associations through selective replacement of microbial taxa. Previous studies in Songnen alkaline grasslands have demonstrated that soil pH and EC are dominant factors controlling bacterial community composition, with different bacterial groups exhibiting distinct responses to environmental stress gradients [29].
Fungal networks showed similar responses to environmental filtering, with pH and EC strongly influencing fungal diversity and community composition. The close relationship between fungal β-diversity and Net property suggests that fungal network assembly was particularly associated with compositional shifts among degradation stages. This stronger dependence on community turnover may reflect the ecological specialization and habitat preferences of fungal taxa. Previous studies in the Songnen Plain have shown that pH, EC, and SOC are important drivers of fungal community assembly, while nutrient availability may differentially influence bacterial and fungal responses [29].
Although vegetation biomass provides important carbon resources for soil microorganisms, it showed limited direct effects on microbial network properties in our SEM models. Under advanced degradation, reduced vegetation cover and intensified soil stress may weaken plant-mediated regulation, causing microbial networks to become increasingly controlled by soil physicochemical constraints and species turnover.
4.5. Ecological Implications and the Potential for Microbial Indicators of Grassland Degradation
Our findings provide important implications for grassland degradation assessment and management. The transition from MD to SD represented a critical stage where microbial diversity and network complexity declined sharply, suggesting that preventing further degradation before this threshold may be important for maintaining soil microbial functioning. Similar threshold-based responses have been reported in degraded alpine ecosystems, highlighting the value of identifying early warning stages for ecosystem management [37].
The contrasting responses of bacterial and fungal communities suggest that fungal characteristics may provide sensitive indicators of degradation status. The progressive decline in fungal diversity and changes in fungal network properties indicate that fungal communities may capture ecological deterioration that is not fully reflected by bacterial responses. Previous studies have also suggested that fungal community characteristics can serve as indicators of soil quality and ecosystem health [42]. In addition, the increased relative representation of Deinococcus–Thermus under extreme degradation suggests its potential as a stress-associated indicator taxon in saline environments [43].
Although network complexity decreased under advanced degradation, the increase in positive associations and clustering indicates that microbial communities may reorganize their interactions under environmental stress. Such network-level responses provide additional information beyond species diversity alone, emphasizing the importance of considering microbial interactions when evaluating ecosystem stability. Previous studies have demonstrated that network structure can influence ecosystem resilience and responses to disturbance [44].
Overall, our study highlights the potential of integrating microbial network properties with traditional diversity-based indicators for grassland degradation assessment. Network metrics, together with community composition and diversity measures, may provide complementary perspectives for evaluating microbial functional stability and ecosystem health [45].
5. Conclusions
Overall, our findings supported the three proposed hypotheses. First, microbial co-occurrence networks exhibited nonlinear responses along the degradation gradient, with network complexity reaching a peak at the moderate degradation stage and collapsing during the transition to severe degradation, confirming that degradation-induced network simplification was most pronounced beyond the ecological threshold. Second, fungal communities showed greater sensitivity to degradation than bacterial communities, as indicated by the continuous decline in fungal diversity and stronger compositional turnover, supporting the hypothesis that fungi are more vulnerable to vegetation loss and environmental stress. Third, soil alkalization and salinization were identified as the primary drivers regulating microbial network changes, while vegetation-mediated effects contributed indirectly through changes in microbial diversity, confirming the proposed environmental filtering mechanism. These results highlight that microbial network restructuring and hub taxa turnover are sensitive responses associated with grassland degradation, providing potential candidates for future development of microbial indicators after further validation across broader spatial and temporal scales.
Supplementary Materials
The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/agriculture16161734/s1. Supplementary Table S1. Key bacterial hub taxa identified across grassland degradation gradient; Supplementary Table S2. Key fungal hub taxa across degradation gradient.
Author Contributions
Conceptualization, G.L. and J.W.; methodology, G.L., D.S. and Z.J.; software, Z.J.; validation, G.L., D.S. and Z.J.; formal analysis, G.L.; investigation, D.S. and Z.J.; resources, B.N.; data curation, G.L. and Z.J.; writing—original draft preparation, G.L.; writing—review and editing, B.N. and J.W.; visualization, Z.J.; supervision, B.N.; project administration, J.W.; funding acquisition, J.W. All authors have read and agreed to the published version of the manuscript.
Funding
This research was funded by the National Natural Science Foundation of China, grant numbers U24A205855, U25A20761 and 42301130. Scientific Research Project of Heilongjiang Ecological Environment Protection, Department of Ecology and Environment of Heilongjiang Province, and the Science (Grant No. HST2024ST007) and Technology Project of the Education Department of Jilin Province (Grant No. JJKH20261186KJ).
Data Availability Statement
The original contributions presented in this study are included in the article. Further inquiries can be directed to the corresponding author.
Conflicts of Interest
The authors declare that they have no known competing financial interests or personal relationships that could have appeared to influence the work reported in this paper.
References
- Gibson, D.J. Grasses and Grassland Ecology; Oxford University Press: Oxford, UK, 2009. [Google Scholar]
- Petermann, J.S.; Buzhdygan, O.Y. Grassland biodiversity. Curr. Biol. 2021, 31, R1195–R1201. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lu, X. Degraded grassland vegetation and soil characteristics: Challenges, opportunities, and sustainable development. Adv. Resour. Res. 2024, 4, 205–220. [Google Scholar]
- Diallo, H.A. United Nations convention to Combat desertification (UNCCD). In Proceedings of the The Future of Drylands: International Scientific Conference on Desertification and Drylands Research Tunis, Tunisia; Springer: Berlin/Heidelberg, Germany, 2006; pp. 13–16. [Google Scholar]
- Brown, C.G. Sustainable development in western China: Managing people, livestock and grasslands in pastoral areas. In Sustainable Development in Western China; Edward Elgar Publishing: Cheltenham, UK, 2008. [Google Scholar]
- Bryan, B.A.; Gao, L.; Ye, Y.; Sun, X.; Connor, J.D.; Crossman, N.D.; Stafford-Smith, M.; Wu, J.; He, C.; Yu, D. China’s response to a national land-system sustainability emergency. Nature 2018, 559, 193–204. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kemp, D.R.; Behrendt, K.; Badgery, W.B.; Han, G.D.; Li, P.; Zhang, Y.; Wu, J.; Hou, F. Chinese degraded grasslands–pathways for sustainability. Rangel. J. 2020, 42, 339–346. [Google Scholar] [CrossRef] [Scilit]
- Li, L.; Chen, J.; Han, X.; Zhang, W.; Shao, C. Meadow Grassland Ecosystem. In Grassland Ecosystems of China: A Synthesis and Resume; Springer: Berlin/Heidelberg, Germany, 2020; Volume 2, pp. 455–514. [Google Scholar]
- Du, Y.; Yang, Y.; Wu, S.; Gao, X.; He, X.; Dong, S. Core microbes regulate plant-soil resilience by maintaining network resilience during long-term restoration of alpine grasslands. Nat. Commun. 2025, 16, 3116. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pedrinho, A.; Mendes, L.W.; de Araujo Pereira, A.P.; Araujo, A.S.F.; Vaishnav, A.; Karpouzas, D.G.; Singh, B.K. Soil microbial diversity plays an important role in resisting and restoring degraded ecosystems. Plant Soil 2024, 500, 325–349. [Google Scholar] [CrossRef] [Scilit]
- Compant, S.; Cassan, F.; Kostić, T.; Johnson, L.; Brader, G.; Trognitz, F.; Sessitsch, A. Harnessing the plant microbiome for sustainable crop production. Nat. Rev. Microbiol. 2025, 23, 9–23. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ravi, R.K.; Balachandar, M.; Yuvarani, S.; Anaswara, S.; Pavithra, L.; Muthukumar, T. Arbuscular mycorrhiza in sustainable plant nitrogen nutrition: Mechanisms and impact. In Soil Nitrogen Ecology; Springer: Berlin/Heidelberg, Germany, 2021; Volume 62, pp. 407–436. [Google Scholar]
- Trivedi, P.; Delgado-Baquerizo, M.; Anderson, I.C.; Singh, B.K. Response of soil properties and microbial communities to agriculture: Implications for primary productivity and soil health indicators. Front. Plant Sci. 2016, 7, 990. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Muscolo, A.; Settineri, G.; Attinà, E. Early warning indicators of changes in soil ecosystem functioning. Ecol. Indic. 2015, 48, 542–549. [Google Scholar] [CrossRef] [Scilit]
- Yuan, X.L.; Zhu, X.T.; Shi, Y.; Miao, Y.; Zhang, R.G.; Li, P.; Shen, C. Soil microbiomes in degraded grasslands: Assembly, function, and application. Grassl. Res. 2025, 4, 352–365. [Google Scholar] [CrossRef] [Scilit]
- Qiao, X.; Yan, X.; Dong, C.; Tao, L.; Aili, A.; Waheed, A. From microbiome collapse to recovery: A roadmap for microbiome-informed grassland restoration under global change. Front. Microbiol. 2026, 17, 1741287. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gralka, M.; Szabo, R.; Stocker, R.; Cordero, O.X. Trophic interactions and the drivers of microbial community assembly. Curr. Biol. 2020, 30, R1176–R1188. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Oña, L.; Shreekar, S.K.; Kost, C. Disentangling microbial interaction networks. Trends Microbiol. 2025, 33, 619–634. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Delmas, E.; Besson, M.; Brice, M.H.; Burkle, L.A.; Dalla Riva, G.V.; Fortin, M.J.; Gravel, D.; Guimarães, P.R., Jr.; Hembry, D.H.; Newman, E.A. Analysing ecological networks of species interactions. Biol. Rev. 2019, 94, 16–36. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Aquilué, N.; Filotas, É.; Craven, D.; Fortin, M.J.; Brotons, L.; Messier, C. Evaluating forest resilience to global threats using functional response traits and network properties. Ecol. Appl. 2020, 30, e02095. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wu, Z.; Cheng, S.; Xu, K.; Qian, Y. Ecological network resilience evaluation and ecological strategic space identification based on complex network theory: A case study of Nanjing city. Ecol. Indic. 2024, 158, 111604. [Google Scholar] [CrossRef] [Scilit]
- Keyes, A.A.; McLaughlin, J.P.; Barner, A.K.; Dee, L.E. An ecological network approach to predict ecosystem service vulnerability to species losses. Nat. Commun. 2021, 12, 1586. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sole, R.V.; Montoya, M. Complexity and fragility in ecological networks. Biol. Sci. 2001, 268, 2039–2045. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tong, A.; Zhou, Y.; Chen, T.; Qu, Z. Constructing an ecological spatial network optimization framework from the pattern–process–function perspective: A case study in Wuhan. Remote Sens. 2025, 17, 2548. [Google Scholar] [CrossRef] [Scilit]
- Wu, Y.; Liang, A.; Ding, M.; Zhang, H.; Xu, H.; Zhang, Y. Meadow degradation reduces microbial β diversity and network complexity while enhancing network stability. Appl. Soil Ecol. 2024, 204, 105733. [Google Scholar] [CrossRef] [Scilit]
- Guo, P.; Guo, W.; Hao, B.; Zhang, Z.; Lu, C.; Liu, T.; Ding, S.; Zhao, L.; Cheng, J.; Li, F.Y. Microbial community in the Leymus chinensis rhizosphere associates with its high production in mild saline–alkaline grassland. Land Degrad. Dev. 2023, 34, 5788–5804. [Google Scholar] [CrossRef] [Scilit]
- Yang, R.; Qi, Z.; Yang, T.; Li, Y.; Xu, L. Distinct bacterial and fungal coexistence patterns and their associations with grassland productivity on the Tibetan Plateau. Agric. Ecosyst. Environ. 2026, 397, 110076. [Google Scholar] [CrossRef] [Scilit]
- Bai, Z.; Jia, A.; Li, H.; Wang, M.; Qu, S. Explore the soil factors driving soil microbial community and structure in Songnen alkaline salt degraded grassland. Front. Plant Sci. 2023, 14, 1110685. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, S.; Sun, L.; Ling, N.; Zhu, C.; Chi, F.; Li, W.; Hao, X.; Zhang, W.; Bian, J.; Chen, L.; et al. Exploring soil factors determining composition and structure of the bacterial communities in saline-alkali soils of Songnen Plain. Front. Microbiol. 2020, 10, 2902. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, M.; Zhang, F.; Xu, J.; Ding, Y.; Zhang, N. Soil microbial community responses to alpine meadow degradation in Maqu: Implications for semi-arid ecosystem restoration. J. Arid. Environ. 2026, 234, 105580. [Google Scholar] [CrossRef] [Scilit]
- Ding, J.; Wang, Y.; Yu, S. Divergent Assembly of Bacteria and Fungi During Saline–Alkali Wetland Degradation. Biology 2025, 15, 61. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Abdelkader, M.S.; Abdalla, S.; Abdelrahman, A.A.; Amin, I.A.; Ramadan, M.; Salah, M. Irrigation water quality shapes soil microbiomes: A 16 S rRNA-based biogeographic study in arid ecosystems. Sci. Rep. 2025, 15, 28460. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Genderjahn, S.; Alawi, M.; Mangelsdorf, K.; Horn, F.; Wagner, D. Desiccation-and saline-tolerant bacteria and archaea in kalahari pan sediments. Front. Microbiol. 2018, 9, 2082. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gao, Y.-C.; Wang, J.-N.; Guo, S.-H.; Hu, Y.-L.; Li, T.-T.; Mao, R.; Zeng, D.-H. Effects of salinization and crude oil contamination on soil bacterial community structure in the Yellow River Delta region, China. Appl. Soil Ecol. 2015, 86, 165–173. [Google Scholar] [CrossRef] [Scilit]
- Telesh, I.; Schubert, H.; Skarlato, S. Life in the salinity gradient: Discovering mechanisms behind a new biodiversity pattern. Estuar. Coast. Shelf Sci. 2013, 135, 317–327. [Google Scholar] [CrossRef] [Scilit]
- Skarlato, S.O.; Telesh, I.V.; Matantseva, O.V.; Pozdnyakov, I.A.; Berdieva, M.A.; Schubert, H.; Filatova, N.A.; Knyazev, N.A.; Pechkovskaya, S.A. Studies of bloom-forming dinoflagellates Prorocentrum minimum in fluctuating environment: Contribution to aquatic ecology, cell biology and invasion theory. Protistology 2018, 12, 113–157. [Google Scholar] [CrossRef] [Scilit]
- Yin, M.; Ye, Y.; Liu, X.; Xiong, W.; Liu, S.; Sun, H.; Sun, W.; Zhang, Y. Divergent Responses of Microbial Networks to Global Change Scenarios during Alpine Cushion Plant Degradation. Plant Divers. 2026, 48, 800–814. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bertness, M.D.; Cavieres, L.A.; Lortie, C.; Callaway, R.M. Positive interactions and interdependence in communities. Trends Ecol. Evol. 2024, 39, 1014–1023. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- He, Q.; Bertness, M.D. Extreme stresses, niches, and positive species interactions along stress gradients. Ecology 2014, 95, 1437–1443. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, F.; Wu, L.; Xu, C.; Guo, S.; Zhao, J.; Wang, Y.; Li, P.; Zhu, B. Virus-inclusive microbial network relationships align with the stress gradient hypothesis in saline-alkali agroecosystems. Soil Biol. Biochem. 2026, 216, 110123. [Google Scholar] [CrossRef] [Scilit]
- Menéndez-Serra, M.; Ontiveros, V.J.; Barberán, A.; Casamayor, E.O. Absence of stress-promoted facilitation coupled with a competition decrease in the microbiome of ephemeral saline lakes. Environ. Microbiol. 2022, 103, e3834. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wu, X.; Yang, J.; Ruan, H.; Wang, S.; Yang, Y.; Naeem, I.; Wang, L.; Liu, L.; Wang, D. The diversity and co-occurrence network of soil bacterial and fungal communities and their implications for a new indicator of grassland degradation. Ecol. Indic. 2021, 129, 107989. [Google Scholar] [CrossRef] [Scilit]
- Hira, P.; Bajaj, A.; Puri, A.; Talwar, C.; Khurana, H.; Negi, R.; Singh, Y.; Lal, R.; Shakarad, M. Microbial genomics and metagenomics in India: Explorations and perspectives. Proc. Indian Natl. Sci. Acad. 2019, 85, 999–1023. [Google Scholar] [CrossRef] [Scilit]
- Gilarranz, L.J.; Rayfield, B.; Liñán-Cembrano, G.; Bascompte, J.; Gonzalez, A. Effects of network modularity on the spread of perturbation impact in experimental metapopulations. Science 2017, 357, 199–201. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cordier, T.; Alonso-Sáez, L.; Apothéloz-Perret-Gentil, L.; Aylagas, E.; Bohan, D.A.; Bouchez, A.; Chariton, A.; Creer, S.; Frühe, L.; Keck, F. Ecosystems monitoring powered by environmental genomics: A review of current strategies with an implementation roadmap. Mol. Ecol. 2021, 30, 2937–2958. [Google Scholar] [CrossRef] [Scilit] [PubMed]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.