


Abstract
The International Code of Zoological Nomenclature provides, under its principle of priority, that a name that has been declared a synonym of an earlier proposed species remains contestable and open to future research. However, as the Code is concerned with nomenclature and not with taxonomic concepts, it places no restrictions on declarations of synonymy, enabling them to be published without supporting evidence. This freedom, which is at the core of the synonymy ‘problem’, contributes to taxonomic inflation and constrains estimates of diversity. From a theoretical perspective, evidence in an unsupported declaration devolves to that of one specimen, the holotype. Furthermore, in the absence of other evidence, the declaration further devolves to one of opinion, with readers left to judge its value based on their knowledge of the declarator. This approach, based on typification, is contrasted with one in which a species exists independently of our perception and is viewable as samples of its local populations. Rather than an arbiter of usage, the holotype then acts only as a referent to its local source population, whose properties define much of the species concept. A worked example of these concepts using data from the planktonic Foraminifera supports the view that evidence of synonymy lies in the source populations of the holotypes.
1. Introduction
That synonymy has long been a problem in taxonomy was shown in Ref. [1] where Hooker’s [2] (p. xiv) ‘chaos of synonymy’ and Strickland’s [3] (p. 129) ‘curse of Babel’ were noted and the reasons underlying use of such pejorative expressions which led to the gestation of the current Code of Zoological Nomenclature were discussed (ICZN, Code) [4]. In it, a declaration of synonymy (ICZN art 23.3) is a statement that unites two nominal taxa under the name determined by the principle of priority (use the earliest available name). A nominal taxon is a concept denoted by an available name, one which is validly based on a name. The Code does not further specify the contents of the statement and inclusion of supporting evidence for unification is left to the author’s judgement. Importantly, the name remains available: there is a validly named type specimen whose status is contestable. Particularly note that the Code deals with naming taxa, not with taxonomic concepts. Thus in a simple declaration of synonymy, a hitherto valid name is demoted to an available but no longer valid name. Evidence is not required because that would involve consideration of taxonomic concepts, which is beyond the scope of the Code.
While it is good scientific practice that the status of a demoted species remains contestable, commonly it generates a stack of historical references to names that have been declared synonymous. In the instance of the Mammalia clade, the stack is monumentally large [5] (Figure 1) and is equally difficult to unravel as names have moved in and out of synonymy in the course of research. This problem is found across biology ([6,7,8,9,10,11,12]) and its importance for estimates of species diversity is plain to see. Consequently, this instability of valid names, as it was two centuries ago, is cause for complaint and has prompted calls for a code to regulate lists of valid species (e.g., [13,14]). However, campaigners for regulation pay little attention to taxonomic procedures that potentially promote instability in species names, particularly the freedom to declare a valid name to be a synonym of an earlier proposed name without citing evidence. Some conceptual issues of such declarations are outlined here with reference to the role of holotypes as objectively named specimens [15] and related to an example from the zooplankton.
Figure 1.
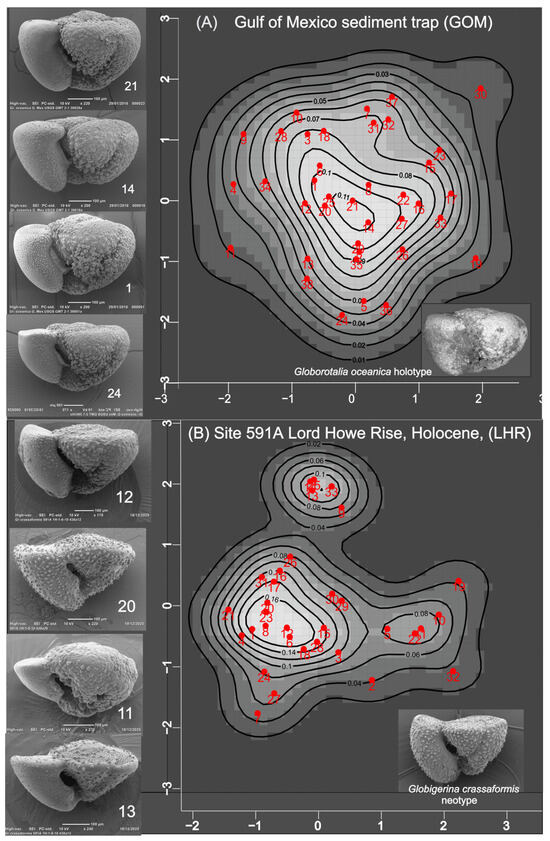
(A) Density map showing probabilities that specimens in the Gulf of Mexico (GOM) sediment trap belong to a normal (Gaussian) shape population. Specimens across the probability range are shown and the inset shows the holotype of Globorotalia oceanica Cushman & Bermudez, 1949. A browser plot of the outline of a selected specimen is available at https://tinyurl.com/altocen2. (B) Density map showing probabilities that specimens in the Southwest Pacific Holocene core sample 1H-1-8-10 cm (LHR) belong to a normal (Gaussian) shape population. Specimens across the probability range are shown and the inset shows the neotype of Globigerina crassaformis Galloway &Wissler, 1927. A browser plot of the outline of a specimen is available at https://tinyurl.com/altocen2.
2. Materials and Methods
Planktonic Foraminifera are a well-researched, globally distributed marine protist clade with an extensive historical record and a taxonomy based largely on their calcitic shells, which preserve valuable environmental signals [16]. The taxonomy of their modern species [17] was revised in Ref. [18], which included a list of synonymous species. For this conceptual review, their designation of Globorotalia oceanica (Cushman & Bermudez, 1949) [19] as a synonym of Globorotalia crassaformis (Galloway & Wissler, 1927) [20] is examined informally, based on my identifications of the taxa.
Gulf of Mexico sediment trap (GOM): This trap is a time series (2008–2012) of foraminiferal and particulate flux at 700 m on the northern Gulf of Mexico continental shelf (27.5° N; 90.3° W; Richey [21]). Tropical Atlantic Central Water is a major component of the upper watermass. Thirty-eight specimens supplied by Caitlin Reynolds were studied from the GMT2-1 sediment trap (212 µm–425 µm fraction); they were collected between 21 and 27 April 2008. This material (Figure 1A) is identified as Globorotalia oceanica.
DSDP Site 591A 1H-1-8-10 cm (LHR): This site (31.35.06°S; 164 26.92° E; 2142 m) is on a southern spur of the eastern part of the Lord Howe Rise in the vicinity of the Tasman Front, a westward-flowing branch of the subtropical East Australian Current. The age of the sample is 9.4 kyr ([22]); 33 specimens were studied from the >149 µm fraction. This material (Figure 1B) is identified as Globorotalia crassaformis.
Methods for collection of morphometric data that capture the specimen shape of the shell in the shown orientation are described in Ref. [23] (Figure 1B). As this trait relates to the trophic and hydrodynamic functions of the organism in a planktonic environment, it is considered to be significant in taxonomic studies. Links to plot the outline of each specimen and the basic data of the analyses are shown in the captions for Figure 1.
3. Species and Their Holotypes
3.1. Realities
Alternative worldviews underlie taxonomy, understood as classification in biology. A nominalist view is that the material of classification is tangible: it can be directly observed. This view is also implicit in some neurovision research in the field of categorization: we build personal concepts of objects as groups, whether or not natural, from direct observation aided by visual recall of known examples. In that view, a species consists of the specimens allocated to it, and no more. In antithesis is the realist view ([15]) that most organisms are intrinsically grouped because of their homeostatic properties [24], which are self-regulating and collectively support the well-being of the organism and aid adaptation to its environment. In that view, the task for classification is not about forming groups, but recognizing them. In biology, this position was promoted by [25], who was influenced by Fisher’s studies of living species [26], and is consistent with the biological species concept [27].
3.2. Applications
How does a declaration of synonymy relate to these worldviews? Where is the evidence that species B-us is a synonym of species A-us? A nominalist might argue that, as their names are objectively attached to their holotypes, their synonymy can be judged from a comparison of these specimens. While few may use that as a sole criterion, in practice it is likely that holotypes have a particular influence on declarations of synonymy because of their authenticity: the names of these specimens cannot be challenged.
Such simple solutions are not available to the realist taxonomist. Although they accept that taxa are natural groups, they can view them only from samples, not in their entirety. To make a judgement of their synonymy, they first must find samples that might come from unitary populations of the taxa (Figure 1). For morphospecies, several steps are suggested. 1. The taxonomist uses their visual perception to select specimens they provisionally identify as A-us or B-us. 2. Morphometric data on a trait present in both groups are gathered. 3. Analyses provide probabilities that specimens belong to unitary populations and the significance of their discrimination. 4. The taxonomist evaluates these statistical grouping data against their knowledge of the functional significance of the trait as a basis for judging whether B-us is a junior synonym of A-us (Figure 2).
Figure 2.
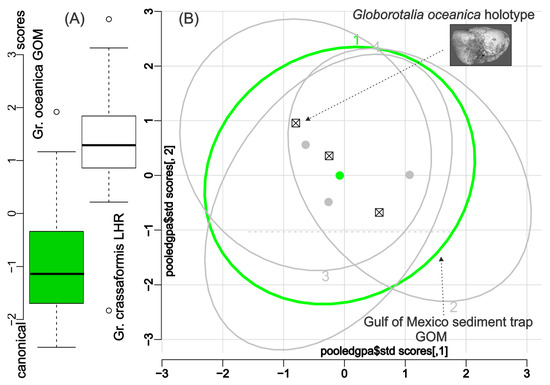
(A) Discrimination of Gulf of Mexico (GOM) sample from Southwest Pacific (LHR) sample. A generalized canonical discriminant analysis (function candisc in R package candisc (available from https://github.com/friendly/candisc/) of data from a multivariate linear model uses PC1:3 projection data from the Procrustes-processed samples. In this analysis, almost all of the between-sample variation is accommodated on one axis, which strongly separates LHR shells from those of GOM. (B) Data ellipses (95% confidence around mean values for a Procrustes analysis; R package shapes (https://cran.r-project.org/web/packages/shapes/index.html) of pooled samples from the Gulf of Mexico (GOM, green), Cariaco Basin (CAR, 2), and Ceara Rise (CER, 3). Sierra Leone Rise (SLR, 4) samples, with the addition of the three named specimens of Globorotalia oceanica. These specimens lie within the confidence limit of each sample. All material is from the source region of Globorotalia oceanica.
In the worked example, Figure 2A shows that all between-sample variation is accommodated on one axis of a generalized multivariate linear model. This is supported by a linear discriminant model, which resolved an overall accuracy of 90%; three GOM specimens were placed in the LHR category. However, these analyses do not address the naming question. Recalling that taxon names are attached to their holotypes, does the analysis establish that the groups recognized in the analysis represent A-us and B-us? How do these names act as referents? Article 23.3 of the Code refers to the unification of taxa, whose only objectively named specimens are the holotypes. A solution based on the view that species taxa are polytypic populations [16] that exist independently of our perception is that the name is tied via the holotype to the local population from which it was sourced. A declaration of synonymy then needs to show that the holotype of the junior synonym falls within the senior synonym’s source population, as sampled. In practice, this sets a high standard of evidence, often difficult to obtain and may require proxy data, as are used in Figure 2B.
4. Discussion
Part of the solution to a problem is to identify its causes. Garnett & et al. [13] support the view that synonymy is indeed a Tower of Babel and recommend that taxonomic commissions be tasked to produce standardized global species lists overseen by a judicial committee. Their monumental proposal provides a solution that would stem the growth of Babel but does not provide a remedy for its principal contributor, here considered to be unsupported declarations of synonymy. While that outlined here is potentially one of several, it is demonstrably operational.
Although Ref. [18] outlines reasons for exclusion of taxa from the list of modern species, for Globorotalia oceanica their only comment is that Ref. [28] considered it extant. As presented, their procedure closely matches a nominalist interpretation of the role of the holotype [15] as an arbiter of usage; although Ref. [18] acknowledges the collaboration of members of the SCOR/IGBP working group 138 in preparing their list, it is likely that data additional to those from the holotypes were considered. Nevertheless, as we are not privy to them, we do not know the basis of their decision about the status of Globorotalia oceanica. In the absence of data, what Ref. [18] provides is expert judgement about its synonymous status.
4.1. The Role of Experts
Expert judgements like those in Ref. [18] on the formal status of species are the modus operandi underpinning taxonomy [7] and, to an unknown extent, contribute to the ‘synonymy overload’ that plagues estimates of diversity. In the absence of data, is their judgement about the synonymous status of Globorotalia oceanica credible? Here, augmentation theory [29], which focuses on the attributes of experts for judging the value of their opinions, is helpful. Potentially applicable are questions [30] (p. 750) to be answered in an appeal to expert opinion, several of which I answer. How credible are Brummer & Kucera (B&K) as an expert source? (ans: highly credible). Are B&K experts in planktonic foraminifera? (ans: yes). Is their decision on Globorotalia oceanica consistent with that of other experts? (ans: yes). Is their decision based on evidence? (ans: limited to the holotypes). Consistent with Ref. [30], a test designed specifically for taxonomy [31] showed that ‘quality of work’ and ‘total productivity’ had the greatest weights when expert opinion was judged. Such reliance may bias how designations of synonymy are assessed and affect, for example, the selection of editors for taxonomic name aggregators like WORMS [32]. Usage ranking [33], a bibliometric approach to mapping synonymy, is similarly hobbled by possible biases in expert opinion, as are estimates of synonymy based on a stochastic flux ratio model [11].
4.2. Test Case—Assessment
Do the morphometric data support the judgement of [18] which, applied to data in Figure 1, would identify both as representing Globorotalia crassaformis? Evidence of a unitary population is clearly defined in Figure 1A, which sampled a living population. Bimodality in Figure 1B is due to a group of elliptically shaped specimens well separated from weakly conical specimens that form the main mode; they are excluded from the following analysis. Canonical discriminant analysis (Figure 2A) of specimens from Figure 1A and from the main mode of Figure 1B shows that it is unlikely that these samples are from a common shape population: the median score for LHR falls close to the maximum score for GOM; the tails of the distributions overlap, as the linear discriminant also shows. Although these data question the judgement of Ref. [18], they are limited to one trait and one dataset. As other spatial/temporal records are neglected, the result is provisional.
Was the referent question posed above answered? Globorotalia oceanica was described from bottom sediment dredged off the northern coast of Cuba and, as the sample was not available, proxy data are used. The site lies under the same tropically sourced watermass as the Caribbean sediment trap (GOM) and three other sites. The data ellipses (Figure 2B) for the four tropical Atlantic–Caribbean samples overlap, with projections for the holotype and paratypes of Globorotalia oceanica positioned within the overlap; this is strong evidence that the name can be applied to these four samples, treated as representing local populations.
5. Conclusions
That the status of a validly proposed taxon is contestable is an essential feature of a science-based taxonomy which should not be impaired by regulation of names. Nevertheless, the freedom allowed by the ICZN to simply declare a taxon to be synonymous with an earlier named taxon, without provision of evidence, contributes to taxonomic instability, does not advance knowledge of taxa, and is an impediment to estimates of diversity. Unsupported declarations represent expressions of expert opinion whose acceptance is shown by augmentation research to be biased in favour of the reputational status of their authors.
The kernel of the problem of unsupported declarations of synonymy is that they implicitly devolve to opinions based on the holotypes (typification), the only objectively named specimens, which are strictly name-bearers and only in a limited sense referents. Reliance on typification contrasts with a realist concept of taxa as composed of sets of local populations. When analyzed, these reveal much about their structure and show that the value of the holotype is no more than the name-bearer from the local population from which it was collected.
Where is the evidence of synonymy? It is primarily in the local populations of the name-bearing specimens, a view that is commonly ignored.
Funding
This research received no external funding.
Data Availability Statement
Source data for the study, are available in folder Atlocenica-data at: https://github.com/GScott170431.
Acknowledgments
I am grateful to Earth Sciences New Zealand for access to facilities and technical support and to M.W. Scott for the plotting application.
Conflicts of Interest
The author declares no conflicts of interest.
References
- Witteveen, J. Suppressing Synonymy with a Homonym: The Emergence of the Nomenclatural Type Concept in Nineteenth Century Natural History. J. Hist. Biol. 2016, 49, 135–189. [Google Scholar] [CrossRef] [Scilit]
- Hooker, J.D. Flora of New Zealand; Lovell Reeve & Co.: London, UK, 1853. [Google Scholar]
- Strickland, H.E. On the Inexpediency of Altering Estabilished Terms in Natural History. Mag. Nat. Hist. J. Zool. Bot. Mineral. Geol. Meteorol. 1837, 1, 127–131. [Google Scholar]
- International Commission on Zoological Nomenclature; Ride, W.D.L.; International Trust for Zoological Nomenclature; Natural History Museum; International Union of Biological Sciences (Eds.) International Code of Zoological Nomenclature: Code International de Nomenclature Zoologique, 4th ed.; International Trust for Zoological Nomenclature, c/o Natural History Museum: London, UK, 1999. [Google Scholar]
- Burgin, C.J.; Zijlstra, J.S.; Becker, M.A.; Handika, H.; Alston, J.M.; Widness, J.; Liphardt, S.; Huckaby, D.G.; Upham, N.S. How Many Mammal Species Are There Now? Updates and Trends in Taxonomic, Nomenclatural, and Geographic Knowledge. J. Mammal. 2025, 106, 1082–1117. [Google Scholar] [CrossRef] [Scilit]
- Alroy, J. How Many Named Species Are Valid? Proc. Natl. Acad. Sci. USA 2002, 99, 3706–3711. [Google Scholar] [CrossRef] [Scilit]
- Garrity, G.M.; Lyons, C. Future-Proofing Biological Nomenclature. OMICS A J. Integr. Biol. 2003, 7, 31–33. [Google Scholar] [CrossRef] [Scilit]
- Kennedy, J. Supporting Taxonomic Names in Cell and Molecular Biology Databases. OMICS A J. Integr. Biol. 2003, 7, 13–16. [Google Scholar] [CrossRef] [Scilit]
- Rao, M.K.V. The Importance of Botanical Nomenclature and Synonymy in Taxonomy and Biodiversity. In Current Science; JSTOR: New York, NY, USA, 2004; Volume 87, pp. 602–606. [Google Scholar]
- Benton, M.J. How to Find a Dinosaur, and the Role of Synonymy in Biodiversity Studies. Paleobiology 2008, 34, 516–533. [Google Scholar] [CrossRef] [Scilit]
- Solow, A.R.; Benton, M.J. On the Flux Ratio Method and the Number of Valid Species Names. Paleobiology 2010, 36, 516–518. [Google Scholar] [CrossRef] [Scilit]
- Mora, C.; Tittensor, D.P.; Adl, S.; Simpson, A.G.B.; Worm, B. How Many Species Are There on Earth and in the Ocean? PLoS Biol. 2011, 9, e1001127. [Google Scholar] [CrossRef] [Scilit]
- Garnett, S.T.; Bánki, O.; Barik, S.K.; Berryman, A.J.; Bouchard, P.; Buckeridge, J.; Christidis, L.; Cigliano, M.M.; Conix, S.; Crawford-Weaver, H.; et al. Measuring the Quality of Species List Governance. BioScience 2026, 76, 254–268. [Google Scholar] [CrossRef] [Scilit]
- Hobern, D.; Barik, S.K.; Christidis, L.; Garnett, S.T.; Kirk, P.; Orrell, T.M.; Pape, T.; Pyle, R.L.; Thiele, K.R.; Zachos, F.E.; et al. Towards a Global List of Accepted Species VI: The Catalogue of Life Checklist. Org. Divers. Evol. 2021, 21, 677–690. [Google Scholar] [CrossRef] [Scilit]
- Scott, G.H. Benchmarking in Taxonomy: The Role of the Holotype. Taxonomy 2025, 5, 62. [Google Scholar] [CrossRef] [Scilit]
- Schiebel, R. Planktic Foraminiferal Sedimentation and the Marine Calcite Budget. Glob. Biogeochem. Cycles 2002, 16, 3-1–3-21. [Google Scholar] [CrossRef] [Scilit]
- Schiebel, R.; Hemleben, C. Planktic Foraminifers in the Modern Ocean; Springer: Berlin/Heidelberg, Germany, 2017. [Google Scholar]
- Brummer, G.-A.; Kučera, M. Taxonomic Review of Living Planktonic Foraminifera. J. Micropalaeontol. 2022, 41, 29–74. [Google Scholar] [CrossRef] [Scilit]
- Cushman, J.A.; Bermudez, P.J. Some Cuban Species of Globorotalia. Contrib. Cushman Lab. Foraminifer. Res. 1949, 25, 26–45. [Google Scholar]
- Galloway, J.J.; Wissler, S.G. Pleistocene Foraminifera from the Lomita Quarry, Palos Verde Hills, California. J. Paleontol. 1927, 1, 35–87. [Google Scholar]
- Richey, J.; Reynolds, C.E.; Tappa, E.; Thunell, R. Weekly Resolution Particulate Flux from a Sediment Trap in the Northern Gulf of Mexico, 2008–2012; USGS Open-File Report 2014–1035; US Geological Survey: Reston, VA, USA, 2014; Volume 9. [Google Scholar]
- Nelson, C.S.; Hendy, C.H.; Cuthbertson, A.M. Compendium of Stable Oxygen and Carbon Isotope Data for the Late Quaternary Interval of Deep-Sea Cores from the New Zealand Sector of the Tasman Sea and Southwest Pacific Ocean; Occasional Report: 16; University of Waikato, Department of Earth Sciences: Hamilton, New Zealand, 1993. [Google Scholar]
- Scott, G.H. Representing Zooplankters: An Example from the Foraminifera. Geosciences 2024, 14, 169. [Google Scholar] [CrossRef] [Scilit]
- Boyd, R. Homeostasis, Species, and Higher Taxa. In Species; Wilson, R.A., Ed.; The MIT Press: Cambridge, MA, USA, 1999. [Google Scholar] [CrossRef] [Scilit]
- Simpson, G.G. Principles of Animal Taxonomy; Columbia University Press: New York, NY, USA, 1961. [Google Scholar] [CrossRef] [Scilit]
- Karlin, S.R.A. Fisher and Evolutionary Theory. Stat. Sci. 1992, 7, 13–33. [Google Scholar] [CrossRef] [Scilit]
- Mayr, E. Principles of Systematic Zoology; McGraw-Hill: Columbus, OH, USA, 1969. [Google Scholar]
- Aze, T.; Ezard, T.H.G.; Purvis, A.; Coxall, H.K.; Stewart, D.R.M.; Wade, B.S.; Pearson, P.N. A Phylogeny of Cenozoic Macroperforate Planktonic Foraminifera from Fossil Data. Biol. Rev. Camb. Philos. Soc. 2011, 86, 900–927. [Google Scholar] [CrossRef] [Scilit]
- Walton, D. Argumentation Theory: A Very Short Introduction. In Argumentation in Artificial Intelligence; Simari, G., Rahwan, I., Eds.; Springer: New York, NY, USA, 2009. [Google Scholar] [CrossRef] [Scilit]
- Walton, D. Examination Dialogue: An Argumentation Framework for Critically Questioning an Expert Opinion. J. Pragmat. 2006, 38, 745–777. [Google Scholar] [CrossRef] [Scilit]
- Caley, M.J.; O’Leary, R.A.; Fisher, R.; Low-Choy, S.; Johnson, S.; Mengersen, K. What Is an Expert? A Systems Perspective on Expertise. Ecol. Evol. 2014, 4, 231–242. [Google Scholar] [CrossRef] [Scilit]
- Vandepitte, L.; Dekeyzer, S.; Decock, W.; Delgat, L.; Boydens, B.; Tyberghein, L.; Vanhoorne, B.; Hernandez, F.; Mees, J.; Horton, T.; et al. The World Register of Marine Species (WoRMS) through the Looking Glass: Insights from the Data Management Team in Light of the Crystal Anniversary of WoRMS. Hydrobiologia 2025, 852, 1–22. [Google Scholar] [CrossRef] [Scilit]
- Huber, R.; Klump, J. Charting Taxonomic Knowledge through Ontologies and Ranking Algorithms. Comput. Geosci. 2009, 35, 862–868. [Google Scholar] [CrossRef] [Scilit]
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the author. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.