


Abstract
The accumulation of biodegradable plastics (BPs) in wastewater treatment plants (WWTPs) presents a novel environmental concern, while carbon deficiency concurrently limits advanced biological denitrification. Herein, this research explored the fate of BPs and their viability as solid-phase carbon donors for denitrification. Six prevalent BPs were selected; results showed that microbially synthesized poly(3-hydroxybutyrate-co-3-hydroxyvalerate) (PHBV) was identified as the optimal solid-phase carbon source with superior DOC bioavailability, achieving a denitrification rate of 0.72 mg/(g·h). Light irradiation and pH variations accelerated DOC release via surface micro-cleavage, predominantly yielding highly active aliphatic oligomers without disrupting the primary polymeric backbone. Furthermore, macromolecular depolymerization genes (cellulase, hexosaminidase) and nitrous oxide reductase genes (nosZ, nosD) were strongly temperature-dependent, which induced the directional enrichment of the core denitrifying genus Thauera and upregulated expression at 25 °C, which promoted NO3− reduction. This research provides the theoretical basis for the in situ resource utilization of BPs for advanced wastewater denitrification.
1. Introduction
As global “plastic bans” and plastic restriction policies continue to be implemented, traditional petrochemical plastics are being rapidly replaced by biodegradable plastics such as polylactic acid (PLA), polyhydroxyalkanoates (PHAs), starch-based materials, and cellulose acetate. Although materials such as PLA and cellulose acetate are widely considered biodegradable, their degradation under environmental conditions is not always complete [1,2]. However, the large-scale production and use of biodegradable plastics (BPs) have given rise to emerging environmental issues related to their accumulation in the environment [3]. Ideally, BPs can be assimilated by microorganisms and completely removed from the environment [4]; however, in real-world water treatment settings, the effective degradation of BPs depends on specific temperature, oxygen conditions, microbial communities, and retention time, and their complete mineralization is often difficult to achieve. Particularly in water treatment systems such as wastewater treatment plants (WWTPs), large quantities of BPs and their fragments are continuously discharged into the effluent in the form of particles or micro-fragments [5]. The environmental behavior and fate of BPs in the effluent system warrant close attention [6].
The inevitable accumulation and gradual breakdown of these BPs in aqueous environments present an unexpected opportunity to repurpose them as slow-release carbon donors. In addition to residual BPs, advanced treatment of effluent still faces limited heterotrophic denitrification due to insufficient carbon sources [7]. The addition of solid-phase carbon sources is a common method for enhancing treatment performance; BPs can release dissolved organic carbon (DOC) in aquatic environments. Compared to natural agricultural wastes, BDPs provide more stable carbon release, demonstrating superior and sustainable denitrification performance for low-C/N wastewater [8], such as polycaprolactone (PCL) and polybutylene succinate (PBS). The carbon-release behavior of BPs is constrained by the inherent physicochemical properties of the materials and external environmental factors [9,10].
BPs of different synthesis types possess entirely distinct molecular backbones, surface hydrophilicities, and degrees of crystallinity. Such structural differences directly determine the susceptibility of internal ester bonds to hydrolysis within the polymers, leading to a fundamental disparity in DOC release rates, carbon source compositions, and bioavailability among different BPs under identical spatiotemporal conditions [9]. Furthermore, environmental conditions are also a key influencing factor. To comprehensively unravel how microbial communities acclimate to BPs as atypical carbon sources, multi-omics approaches have been increasingly deployed. Temperature not only alters the physical hydrolysis and photoaging processes of BP macromolecular segments from a thermodynamic perspective, but also directly affects the composition and function of microbial communities [11]. Their findings revealed that upon assimilation of this highly active DOC, the microbial tricarboxylic acid (TCA) cycle and the synthesis pathways of amino acids and nucleotides are significantly upregulated [12]. This direct acceleration of bacterial ATP synthesis and cell turnover mediated by BPs unleashes the metabolic potential of microorganisms and triggers a significant “pre-excitation effect” in the local microhabitat, which facilitates the directional enrichment of functional microorganisms from specific phyla (such as Proteobacteria, a dominant clade in denitrification) [13].
Previous studies have highlighted the feasibility of using PHBV as a solid-phase carbon source [14]; however, the comprehensive linkage between abiotic environmental aging (pH, light) and the subsequent temperature-driven microbial responses remains poorly understood. Therefore, this study aims to elucidate the temperature-dependent microbial ecological succession and functional network expressions. Specifically, this study conducts the following investigations: (1) it systematically evaluates the carbon release characteristics of common BPs and their potential to promote heterotrophic denitrification as in situ carbon sources; (2) it focuses on PHBV as a model BP material and systematically investigates the effects of abiotic environmental factors, such as pH and light, on the carbon release kinetics and DOM compositional characteristics; (3) it elucidates the temperature-dependent microbial carbon assimilation and nitrogen transformation pathways derived from BPs. The results of this research might provide a solid theoretical foundation for in situ carbon source substitution and low-carbon enhancement technologies in the process of advanced denitrification of effluent.
2. Materials and Methods
2.1. Materials
Six commercially available BPs were selected as solid-phase carbon sources and biofilm carriers in this study, including Poly 3-hydroxybutyrate-co-3-hydroxyvalerate (PHBV), polyhydroxyalkanoates (PHAs), polycaprolactone (PCL), polybutylene adipate-co-terephthalate (PBAT), polybutylene succinate (PBS), and polylactic acid (PLA). All BP materials used in this study were commercially purchased in standard commercial extrusion grades (without functionalization or compounding additives) from Shenzhen eSUN Industrial Co., Ltd. (Shenzhen, China) and were of high purity (>99%). Since DOC release is strongly dependent on the initial exposed surface area, a strict standardization procedure was applied to eliminate size-induced variations. Prior to the experiments, all bulk BPs were uniformly cut, mechanically sieved, and sorted to obtain standard granules (d = 3–4 mm). The granules were then rinsed with ultrapure water and dried. The detailed specifications of each polymer are summarized in Table S1.
2.2. Carbon Source Release and Driving Factor Experiment
2.2.1. Carbon Release Experiments
To systematically quantify the intrinsic carbon release capacity of the different BPs, static batch leaching experiments were conducted. A total of 5.0 g of each BP was added in 250 mL Erlenmeyer flasks containing 200 mL of distilled water, and the flasks were incubated in the dark at 25 ± 1 °C. Over the 25-day experimental period, water samples were collected at 24 h intervals for DOC analysis, and an equal volume of fresh distilled water was immediately added to maintain a constant system volume.
2.2.2. Nitrate Removal Kinetics Experiments
To evaluate the biological denitrification potential, independent sequential batch experiments were performed. Briefly, the batch reactors were inoculated with washed denitrifying activated sludge (obtained from the anoxic tank of a local wastewater treatment plant) and synthetic wastewater. The systems were maintained under strict anoxic conditions by purging with N2 gas (DO < 0.5 mg/L) and incubated in a thermostatic shaker at 25 °C and 135 r/min. For NO3−-N removal kinetics, samples were taken every 30 min over a 12 h period, and all treatments were performed in triplicate.
2.2.3. Driving Factors of Carbon Source Release Experiment
BP (PHBV) with optimal carbon release ability was selected to investigate the effects of light irradiation conditions (light, dark) and pH (3, 7 and 10) on their carbon release characteristics. Flasks containing identical solutions but without BPs were used in parallel as blank controls. The initial pH of the solutions was adjusted to the target values using 0.1 M HCl or 0.1 M NaOH.
The surface morphological evolution of the PHBV particles was observed via scanning electron microscopy (SEM, TESCAN, BrnoBrno, Czech Republic). Prior to imaging, the samples were dried and sputter-coated with a thin layer of gold to enhance conductivity. The imaging was conducted using a secondary electron (SE) detector at an accelerating voltage of 10 kV and a working distance of approximately 10 mm. Modifications in surface functional groups and the polymeric backbone were identified using Fourier transform infrared spectroscopy (FT-IR, Nicolet IS50, Thermo Fisher Scientific, Waltham, MA, USA). The samples were prepared using the potassium bromide (KBr) pellet method, where approximately 2 mg of the dried sample was mixed with 100 mg of KBr and pressed into a transparent pellet. The transmission spectra were recorded over the wavenumber range of 4000–400 cm−1 with a spectral resolution of 4 cm−1 and 32 scans per sample. The Dissolved Organic Matter (DOM) released by BPs was characterized using a UV-visible spectrophotometer (UV-2600, Shimadzu, Kyoto, Japan). Optical indices, including SUVA254, E2/E3, E3/E4, and A253/A203 were calculated to systematically evaluate the molecular weight, aromaticity, and structural evolution of the released carbon. The composition of DOM before and after the experiment was analyzed using a liquid chromatography–mass spectrometry system (LC-MS, Vanquish UHPLC coupled with a QE-HF-X mass spectrometer, Thermo Fisher Scientific, Waltham, MA, USA). Chromatographic separation was performed on a Waters BEH C18 column (2.1 × 100 mm, 1.7 μm). The mobile phase consisted of 0.1% formic acid aqueous solution (A) and methanol (B) at a flow rate of 0.3 mL/min. The mass spectrometer was operated in electrospray ionization negative (ESI-) mode with a full scan range of m/z 100–1000 to enable the detection of highly reactive intermediate metabolites.
2.3. Microbial Ecological Response to Temperature Variations
To investigate the microbial ecological response to seasonal variations, sequential batch reactor (SBR) experiments were executed under three distinct temperature gradients (5 °C, 15 °C, 25 °C). The tail water was prepared following the method of Du, characterized by a low carbon-to-nitrogen (C/N) ratio of 2.0; the concentration of Chemical Oxygen Demand (COD), NO3−-N and PO43−-P were 40 mg/L, 20 mg/L and 2.0 mg/L, respectively. The triplicate sequential batch reactors (SBRs) with a working volume of 1.0 L, amended with 5.0 g of PHBV and activated sludge, were continuously fed with simulated tail water. The systems were operated with a hydraulic retention time (HRT) of 2 days, and the Mixed Liquor Suspended Solids (MLSS) was maintained at approximately 1500 mg/L.
2.4. 16S rRNA Gene Amplicon Sequencing and Functional Prediction
The Fast DNA® Spin Kit for Soil (MP Biomedicals, Irvine, CA, USA) was used to extract genomic DNA from SBR systems at different temperatures (5, 15, 25 °C). The V3–V4 hypervariable regions of the bacterial 16S rRNA gene were amplified utilizing the universal primer pair 338F and 806R. The PCR cycling conditions consisted of an initial denaturation at 95 °C for 3 min, followed by 27 cycles of denaturation at 95 °C for 30 s, annealing at 55 °C for 30 s, and extension at 72 °C for 45 s, with a final extension at 72 °C for 10 min. The purified amplicons were sequenced on an Illumina MiSeq platform, and raw data were processed using the QIIME2 pipeline (version 2022.2). To further decode the functional networks of the microbial communities, specifically regarding macromolecular depolymerization and downstream nitrogen cycling pathways, metagenomic functional prediction was conducted using PICRUSt2 (version 2.3.0_b). The predicted functional genes were annotated against the Kyoto Encyclopedia of Genes and Genomes (KEGG) database.
2.5. Statistical Analysis
All batch experiments and instrumental analyses were executed in independent triplicates, with the macroscopic and molecular results presented as the mean ± standard deviation. Data visualization and bioinformatics heatmap generation were executed utilizing Origin 2021 and specific packages in R software (version 4.2.1), including ggplot2 (version 3.4.0) for data visualization and vegan (version 2.6-4) for community ecological analysis.
3. Results and Discussion
3.1. Carbon Release Characteristics and Denitrification Kinetics of BPs
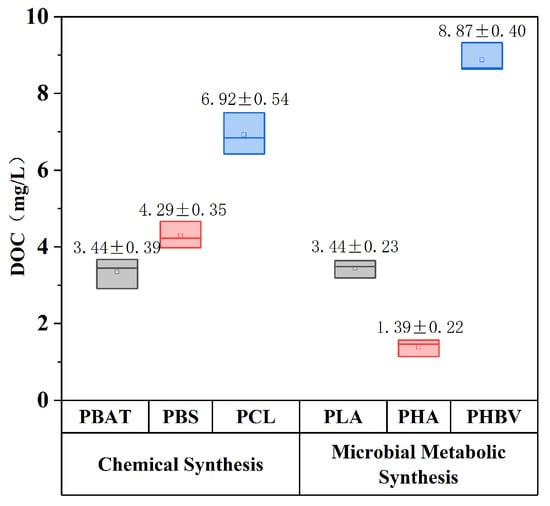
The concentration of DOC released by different kinds of BPs are presented in Figure 1. The DOC releasing content of PHBV (8.87 ± 0.40) was significantly higher than that of the others. This pronounced carbon release from PHBV is attributed to its bio-based molecular backbone, which shares structural homology with natural microbial storage polymers, making its ester bonds highly susceptible to abiotic physical hydrolysis and the subsequent dissolution of soluble low-molecular-weight oligomers from the polymer surface [15]. However, it should be noted that the 25-day carbon release experiments were conducted in distilled water without sterilization; hence, the observed DOC release reflects a combined effect of abiotic hydrolysis and potential incidental microbial degradation, rather than purely abiotic processes.
Figure 1.
The concentration of dissolved organic carbon (DOC) released by biodegradable plastics (BPs).
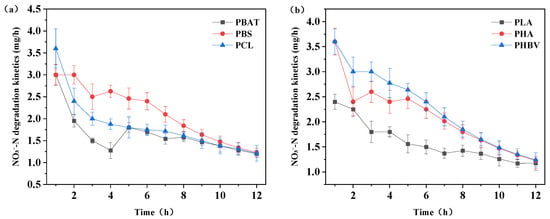
The utility of a solid-phase carbon source lies in the bioavailability of its released DOC to drive heterotrophic denitrification [16]. Figure 2 presents the NO3−-N degradation kinetics of BPs over a 12 h reaction cycle. The kinetic profiles universally exhibited a biphasic pattern: an initial rapid degradation phase (0–6 h) driven by the abundance of readily available surface organic matter, followed by a deceleration phase (6–12 h) governed by the diffusion-limited hydrolysis of the polymer matrix [17]. Specifically, within the microbial metabolic synthesis group (Figure 2b), PHBV achieved a peak initial NO3−-N degradation rate 0.72 mg/(g·h). Among the four BPs evaluated, PHBV and PCL exhibited comparable DOC release and NO3−-N degradation performance in the initial screening. For the subsequent mechanistic investigations, we selected PHBV as the model BP material, as PHBV is one of the most extensively studied and well-characterized solid-phase carbon sources in denitrification applications, and has greater commercial availability and lower production cost than PCL, which favors its practical engineering application.
Figure 2.
NO3−-N degradation kinetics of BPs: (a) chemically synthesized BPs (PBAT, PBS, and PCL); (b) microbially synthesized BPs (PLA, PHA, and PHBV).
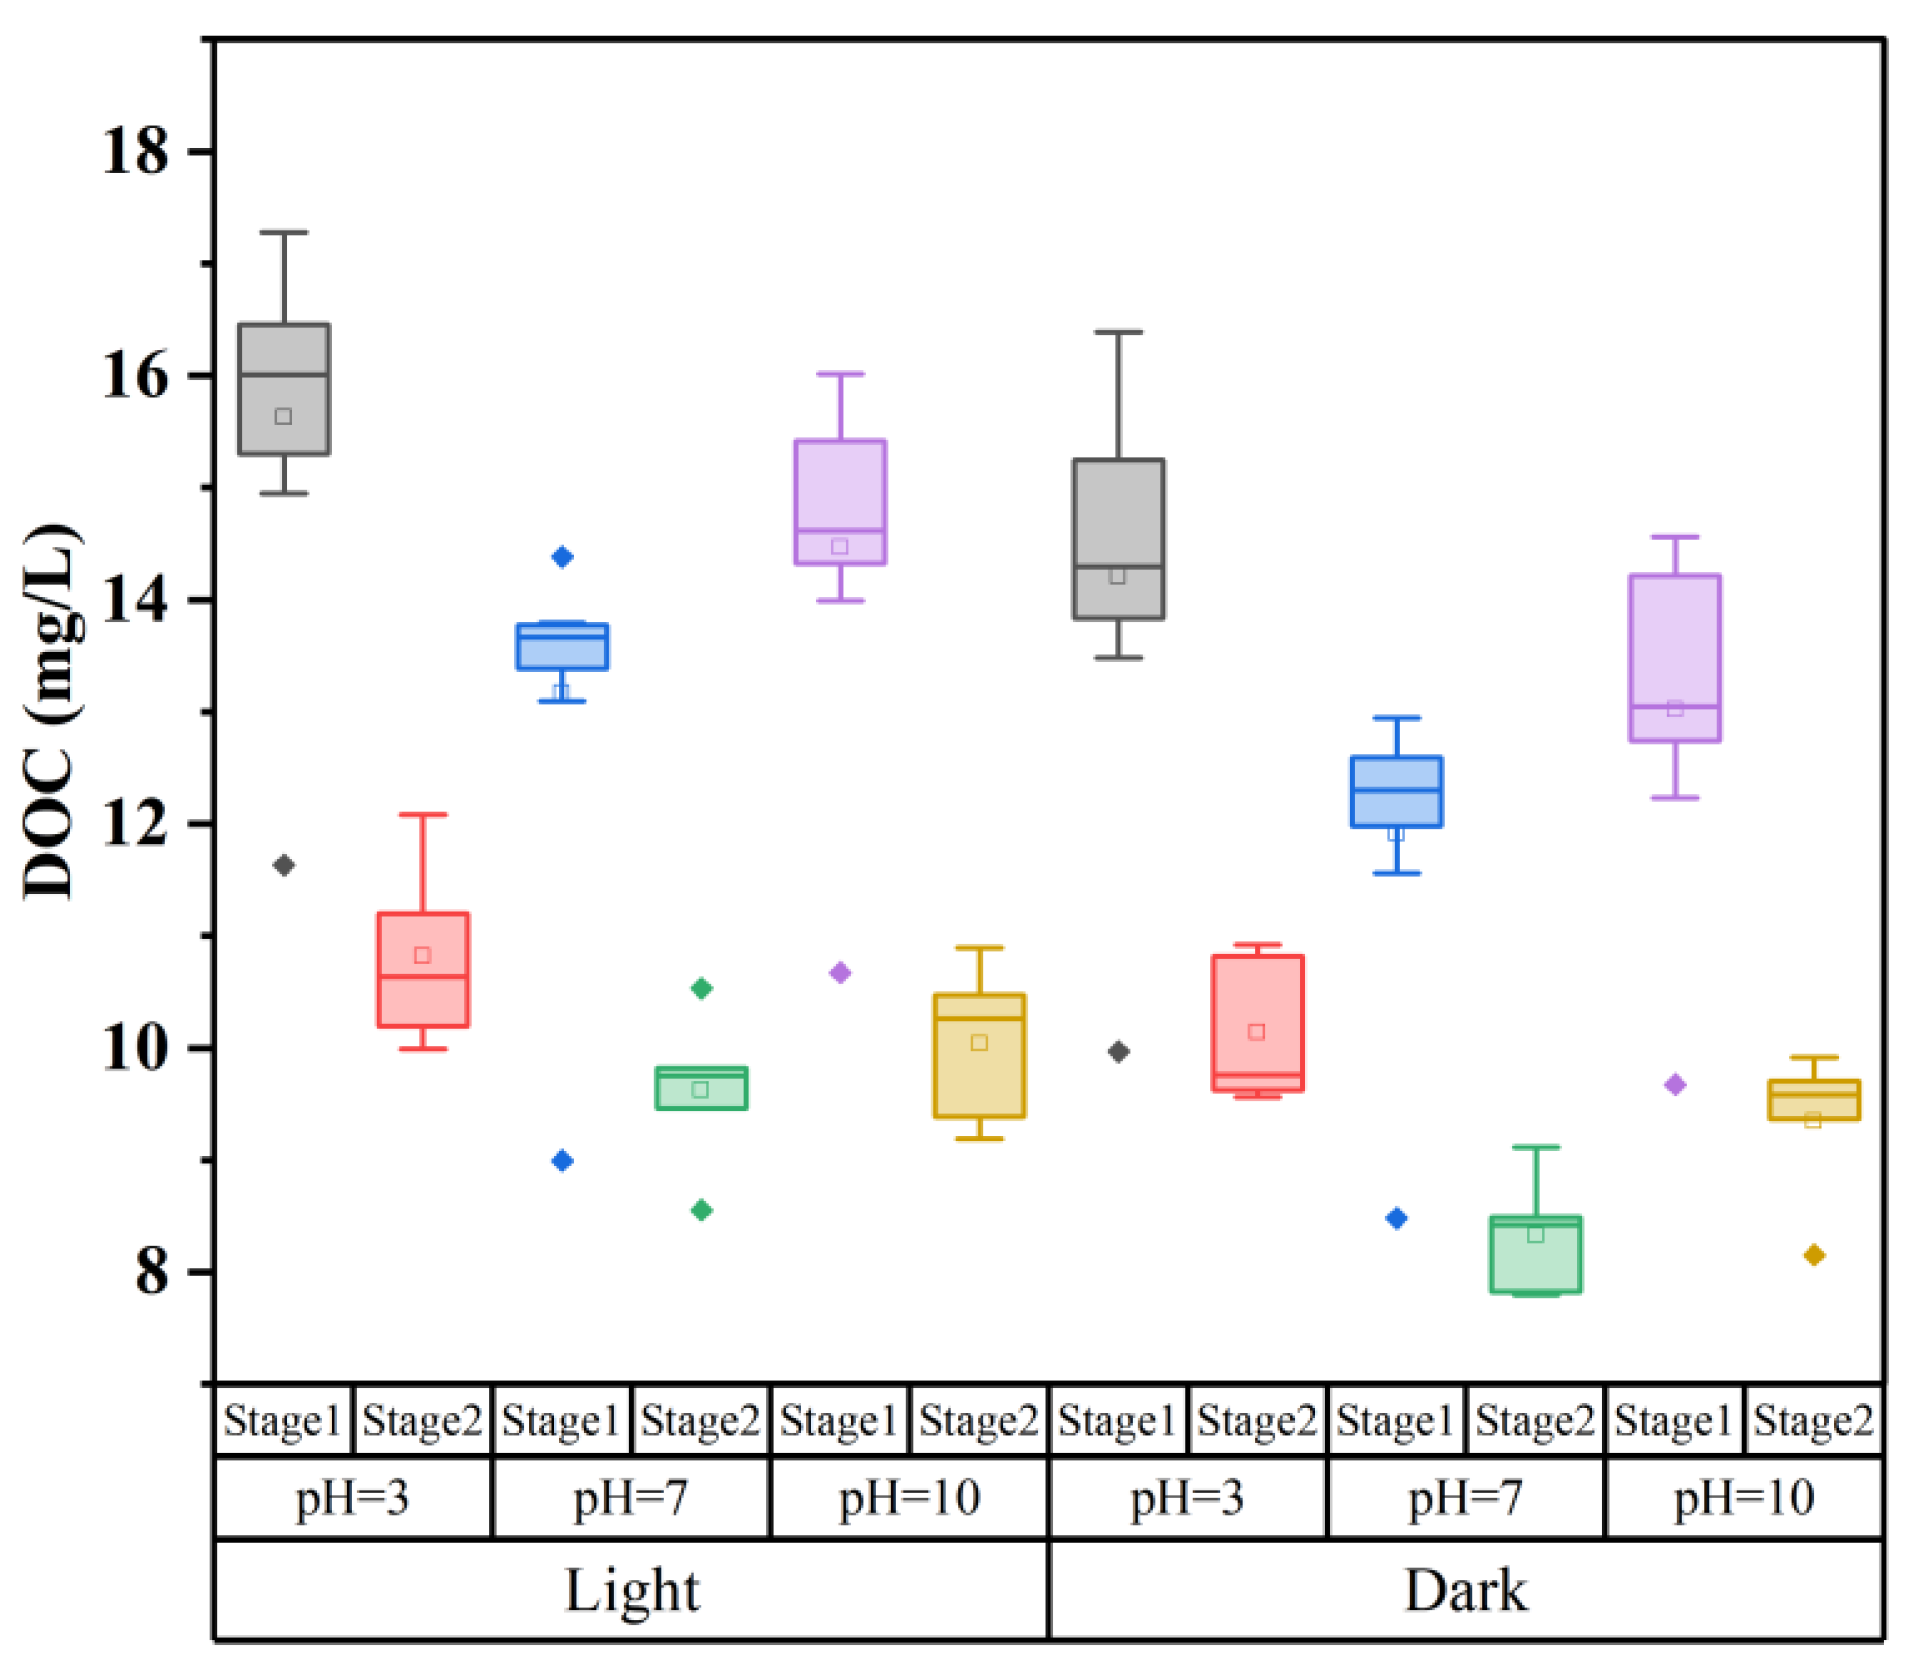
To elucidate the environmental fate and carbon release mechanisms of PHBV under variable aquatic conditions, the abiotic impacts of pH and light irradiation were investigated. Light exposure significantly accelerated the release of DOC from PHBV (Figure 3); under light exposure, the amount of DOC released was 1.1 times that under dark conditions [18]. This accelerated release is primarily attributed to photochemical aging, in which photon energy triggers radical reactions and promotes microcracking on the polymer chain surface [11]. In addition, pH changes significantly affected DOC release, showing a trend of pH = 3 > pH = 10 > pH = 7. Both acidic and alkaline pH conditions effectively catalyzed the hydrolysis of ester bonds on the PHBV surface, accelerating the dissolution of low-molecular-weight organic compounds [9,19,20].
Figure 3.
Effects of light irradiation and pH on DOC release from PHBV across different reaction stages. The distinct colors of the boxplots visually differentiate the specific combinations of pH and reaction stages corresponding to the x-axis labels.
3.2. Structural Characterization of PHBV and Composition Analysis of Released DOC
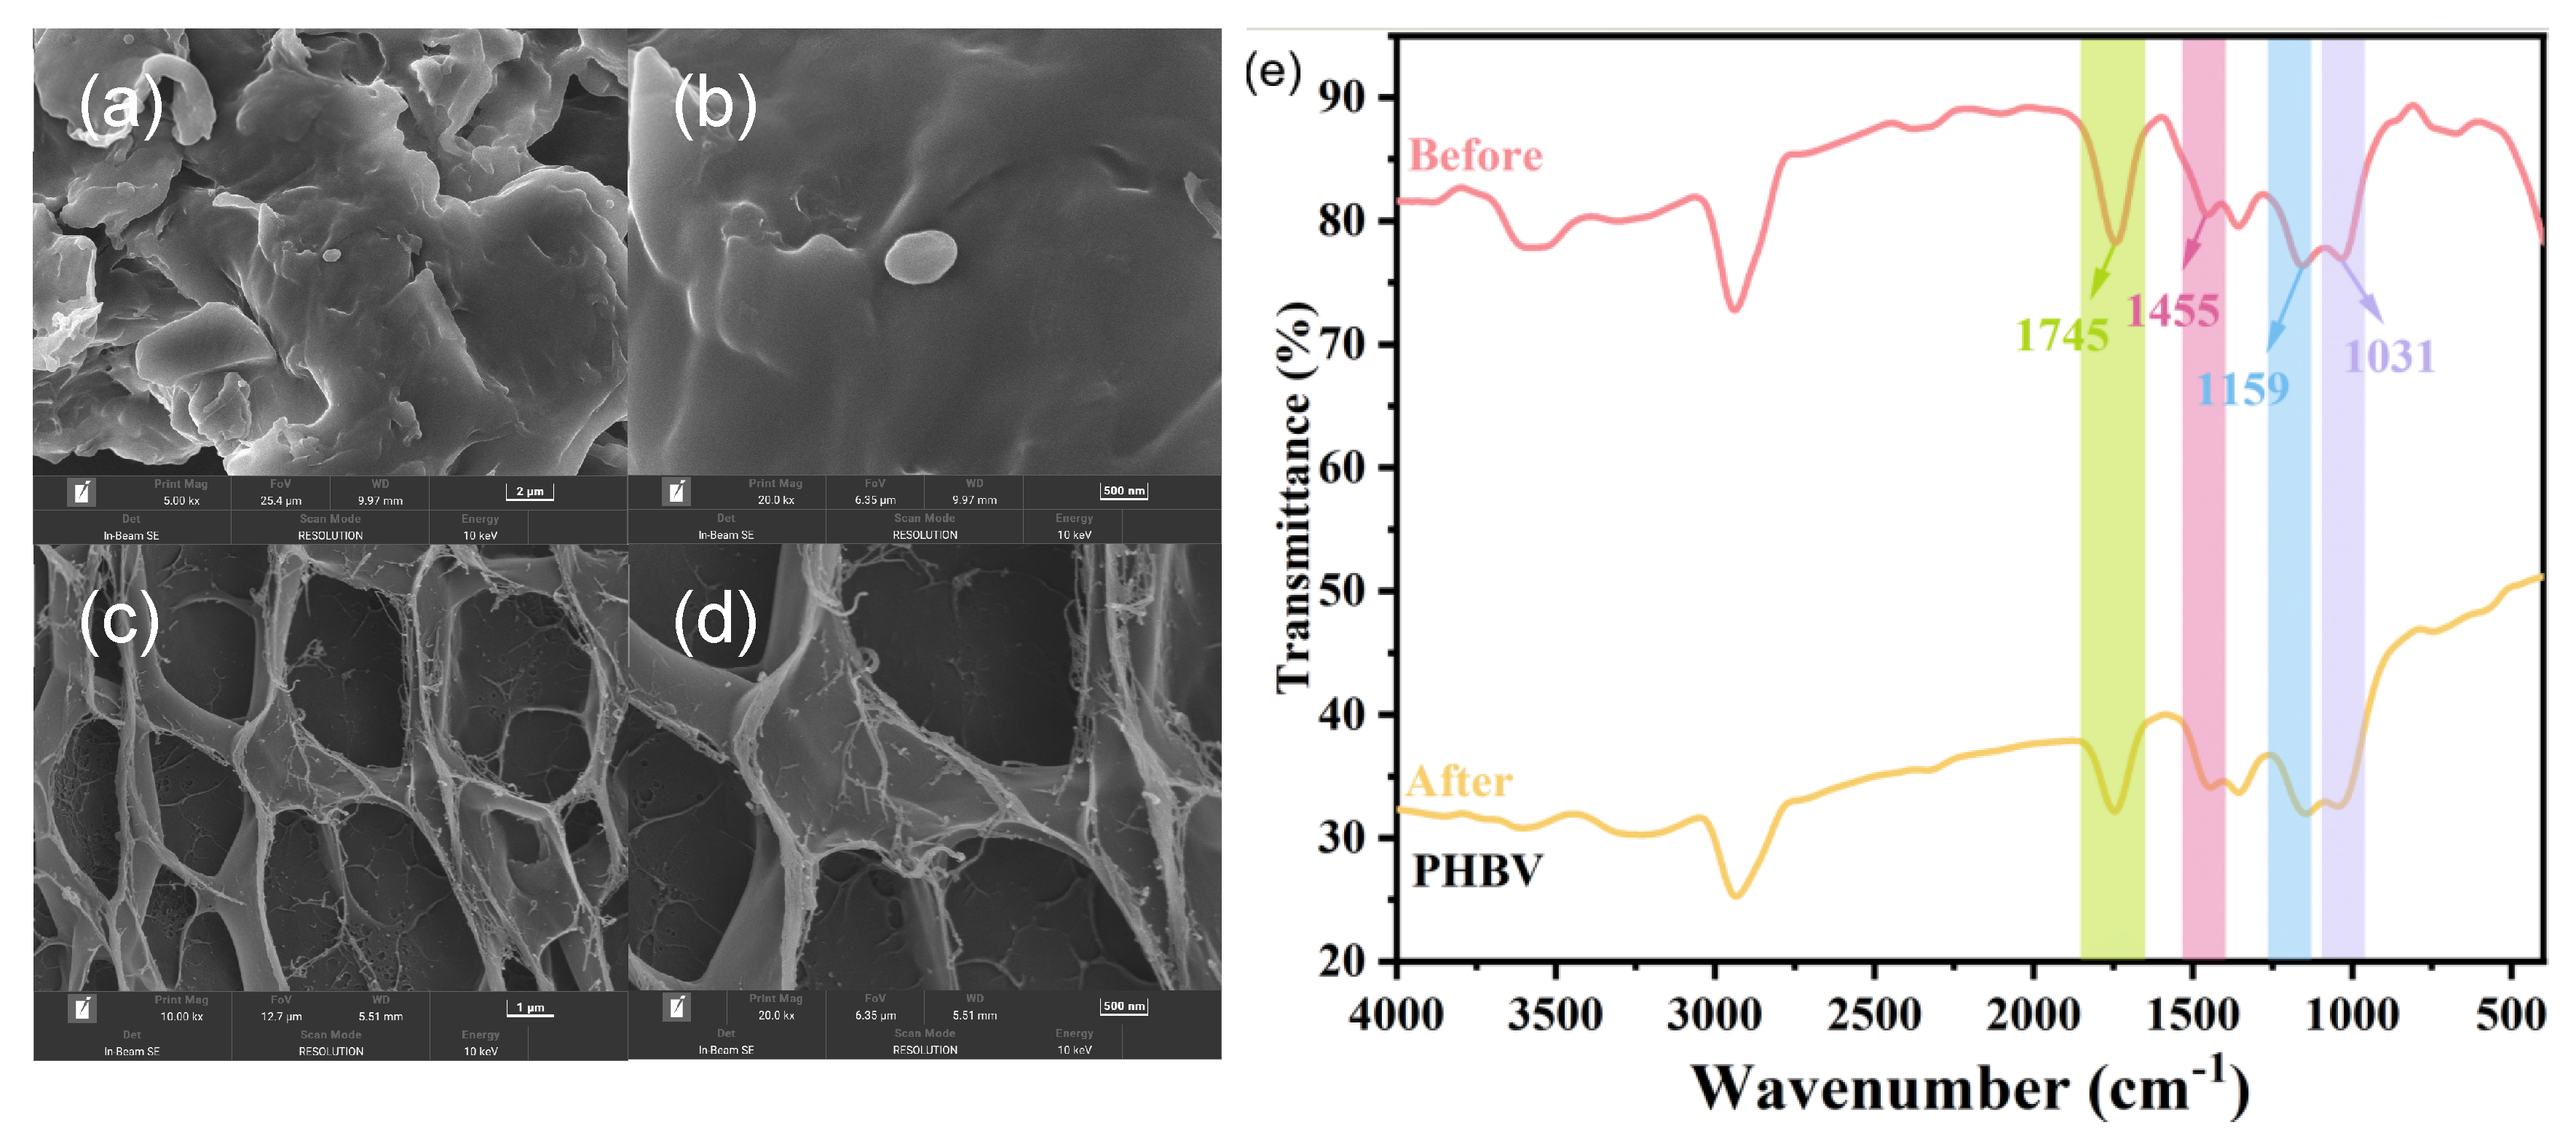
SEM images showed that the initial surface of PHBV was relatively smooth (Figure 4a,b); after microbial degradation, pits and pores appeared on the surface of PHBV (Figure 4c,d). These morphological changes are consistent with surface erosion patterns commonly observed during polymer biodegradation, although SEM alone cannot distinguish between biotic degradation and abiotic physical weathering. The FTIR spectra of PHBV underwent significant changes before and after hydrolysis (Figure 4e). The untreated sample exhibited a distinct ester group C=O stretching vibration peak at 1745 cm−1, a peak at 1455 cm−1 corresponding to —CH2 bending vibration at 1455 cm−1, while the absorption peaks at 1159 cm−1 and 1031 cm−1 can be attributed to C–O–C and C–O stretching vibrations, respectively. The presence of these characteristic peaks suggests that the ester bond structure in the PHBV main chain was largely intact prior to degradation. After hydrolysis, the peak intensities at the aforementioned characteristic peaks in the sample were generally weakened; in particular, the carbonyl peak at 1745 cm−1 and the C–O-related peaks at 1159/1031 cm−1 showed more pronounced attenuation. This spectral attenuation is indicative of ester bond cleavage within the PHBV molecular chains, consistent with the hydrolysis of the polymer backbone [21]. However, it should be noted that FTIR peak intensity changes may also be influenced by surface crystallinity variations or loss of low-molecular-weight oligomers; thus, these spectral data provide supporting evidence for, rather than definitive proof of, backbone cleavage. Concurrently, the changes in absorption in the high-wavenumber region of the spectrum may suggest the introduction of oxygen-containing functional groups onto the PHBV surface, which would be consistent with surface oxidation and increased hydrophilicity [22].
Figure 4.
Structural characterization of PHBV before and after the carbon release process: (a–d) SEM images, (e) FT-IR spectra.
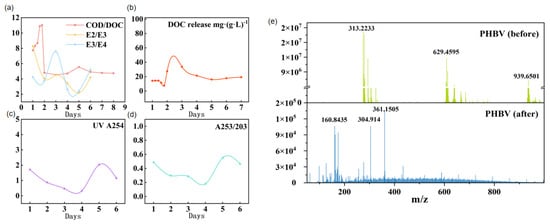
To reveal the compositional characteristics of the DOM released by PHBV, the leachate was analyzed using UV-visible absorption spectroscopy. The UV-visible absorption analysis yielded SUVA254 values in the range of 0.327−2.03 (Figure 5c), along with E2/E3 ratios of 2.19−8.29 and E3/E4 ratios of 2.42−7.6 (Figure 5a). These parameter ranges are consistent with a DOM composition enriched in aliphatic oligomers and monomers, as lower SUVA254 values (<3) are typically associated with low aromaticity in freshwater DOM studies [23]. However, it should be noted that these optical indices provide qualitative, rather than quantitative, information regarding DOM structural characteristics. The A253/A203 ratio (Figure 5d), which has been used in some studies as an indicator of the relative abundance of aromatic versus aliphatic structures [24], similarly offers only indirect structural inference. Collectively, these optical data are consistent with the predominance of aliphatic species in the PHBV leachate.
Figure 5.
Characterization and composition analysis of dissolved organic matter (DOM) released from PHBV: (a) COD/DOC, E2/E3 and E3/E4 ratios; (b) DOC release dynamics; (c) UV254 absorbance; (d) A253/A203 ratio; (e) LC-MS before and after the reaction.
LC-MS analysis provided direct molecular-level information on the DOM components released from PHBV in aqueous systems (Figure 5e). In the leachate from the early stages of the reaction, a series of mass spectrometry peaks in the m/z range of 300–1000 (m/z 313.22, 629.45, 939.65) were detected. These high-m/z signals are tentatively assigned to polymer fragments released during the initial dissolution of PHBV or to residual additives/oligomers from the material synthesis process. In the later stages, high-resolution mass spectrometry detected an increased abundance of small-molecule products (m/z < 300), including peaks consistent with short-chain fatty acids and their oxidized derivatives (e.g., peaks at m/z 89.05, 117.06, and 131.07, which are compatible with acetate, propionate, and their hydroxylated analogues). These small-molecule products are consistent with the degradation pathways of aliphatic polyesters reported in previous literature [15]. However, we emphasize that LC-MS alone cannot distinguish between abiotic hydrolysis products and microbially mediated transformation intermediates without complementary enzymatic or isotopic tracing experiments. We therefore hypothesize that these products may represent highly oxidized short-chain aliphatic intermediates produced by the cleavage of the PHBV carbon backbone under the action of extracellular depolymerases, a hypothesis that warrants verification through future targeted metabolomics studies. In addition, the mass spectrum still shows residual peaks in the 450–950 m/z range, suggesting the presence of some higher-molecular-weight fragments that have not been completely depolymerized [9]. The low UV254 absorbance (stabilizing at ~0.1 by the end of the experiment; Figure 5c) is consistent with the absence of significant conjugated C=C double-bond structures in the released DOM [7,23], which is in agreement with the aliphatic nature of PHBV-derived products, but does not independently confirm the complete absence of all unsaturated species.
3.3. Temperature-Driven Microbial Community Diversity
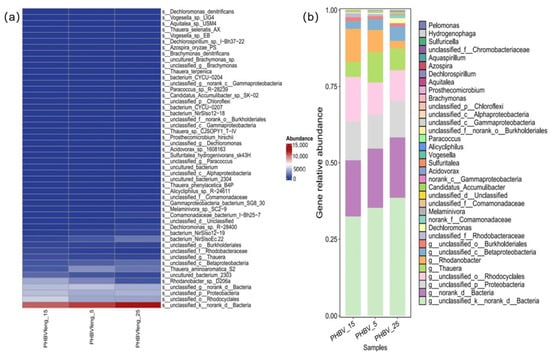
As illustrated in the genus-level relative abundance profiles (Figure 6b), the absolute dominant basal microbial consortia across multiple temperature gradients were primarily composed of Proteobacteria and Rhodocyclales. These primary taxa maintained a high baseline abundance over a broad temperature range from 5 °C to 25 °C. This indicates that PHBV serves not merely as a sustained carbon donor, but its stable three-dimensional polymeric backbone also provides a highly resilient colonization microenvironment, effectively buffering the physical structure of the biofilm against environmental temperature fluctuations [13].
Figure 6.
Microbial community analysis of PHBV under different temperatures. (a) Heatmap analysis of the dominant bacterial genera. (b) Relative abundance of microbial communities at the genus level.
However, temperature variations significantly reshaped the fine-scale structure and metabolic abundance of key functional denitrifying consortia. In conjunction with the taxonomic heatmap (Figure 6a), the enrichment characteristics of specific nitrogen-removal functional groups exhibited temperature dependence. Notably, under the optimal temperature of 25 °C, the relative abundance of Thauera, a classical and highly efficient heterotrophic denitrifying genus, increased significantly. The genus Thauera possesses a robust capacity for extracellular polymer degradation, a broad utilization spectrum for organic carbon sources (particularly short-chain fatty acids), and a complete denitrifying electron transport chain [12]. At 25 °C, the highly reactive aliphatic oligomers released via the accelerated micro-hydrolysis of the PHBV surface provided exceptionally compatible, high-quality electron donors for Thauera, enabling it to rapidly secure a dominant ecological niche during competitive growth. From the fundamental perspective of micro-ecological succession, this enrichment of the core denitrifying genus definitively elucidates the macroscopic denitrification rate peak observed at 25 °C in the preceding kinetic experiments [25]. Conversely, under low-temperature stress at 5 °C and 15 °C, the physical hydrolytic carbon release rate of PHBV declined, and the proliferation of mesophilic efficient denitrifiers such as Thauera was simultaneously suppressed [26,27,28]. This dual inhibition resulted in a marked deterioration of the metabolic coupling efficiency between the electron donor supply and the downstream nitrogen reduction acceptors [13]. In summary, PHBV serves as an effective physical carrier, and its highly bioavailable DOM can precisely induce the directional enrichment of core denitrifying taxa such as Thauera under suitable temperature conditions.
3.4. PHBV-Driven Microbial Community Dynamics and Functional Networks
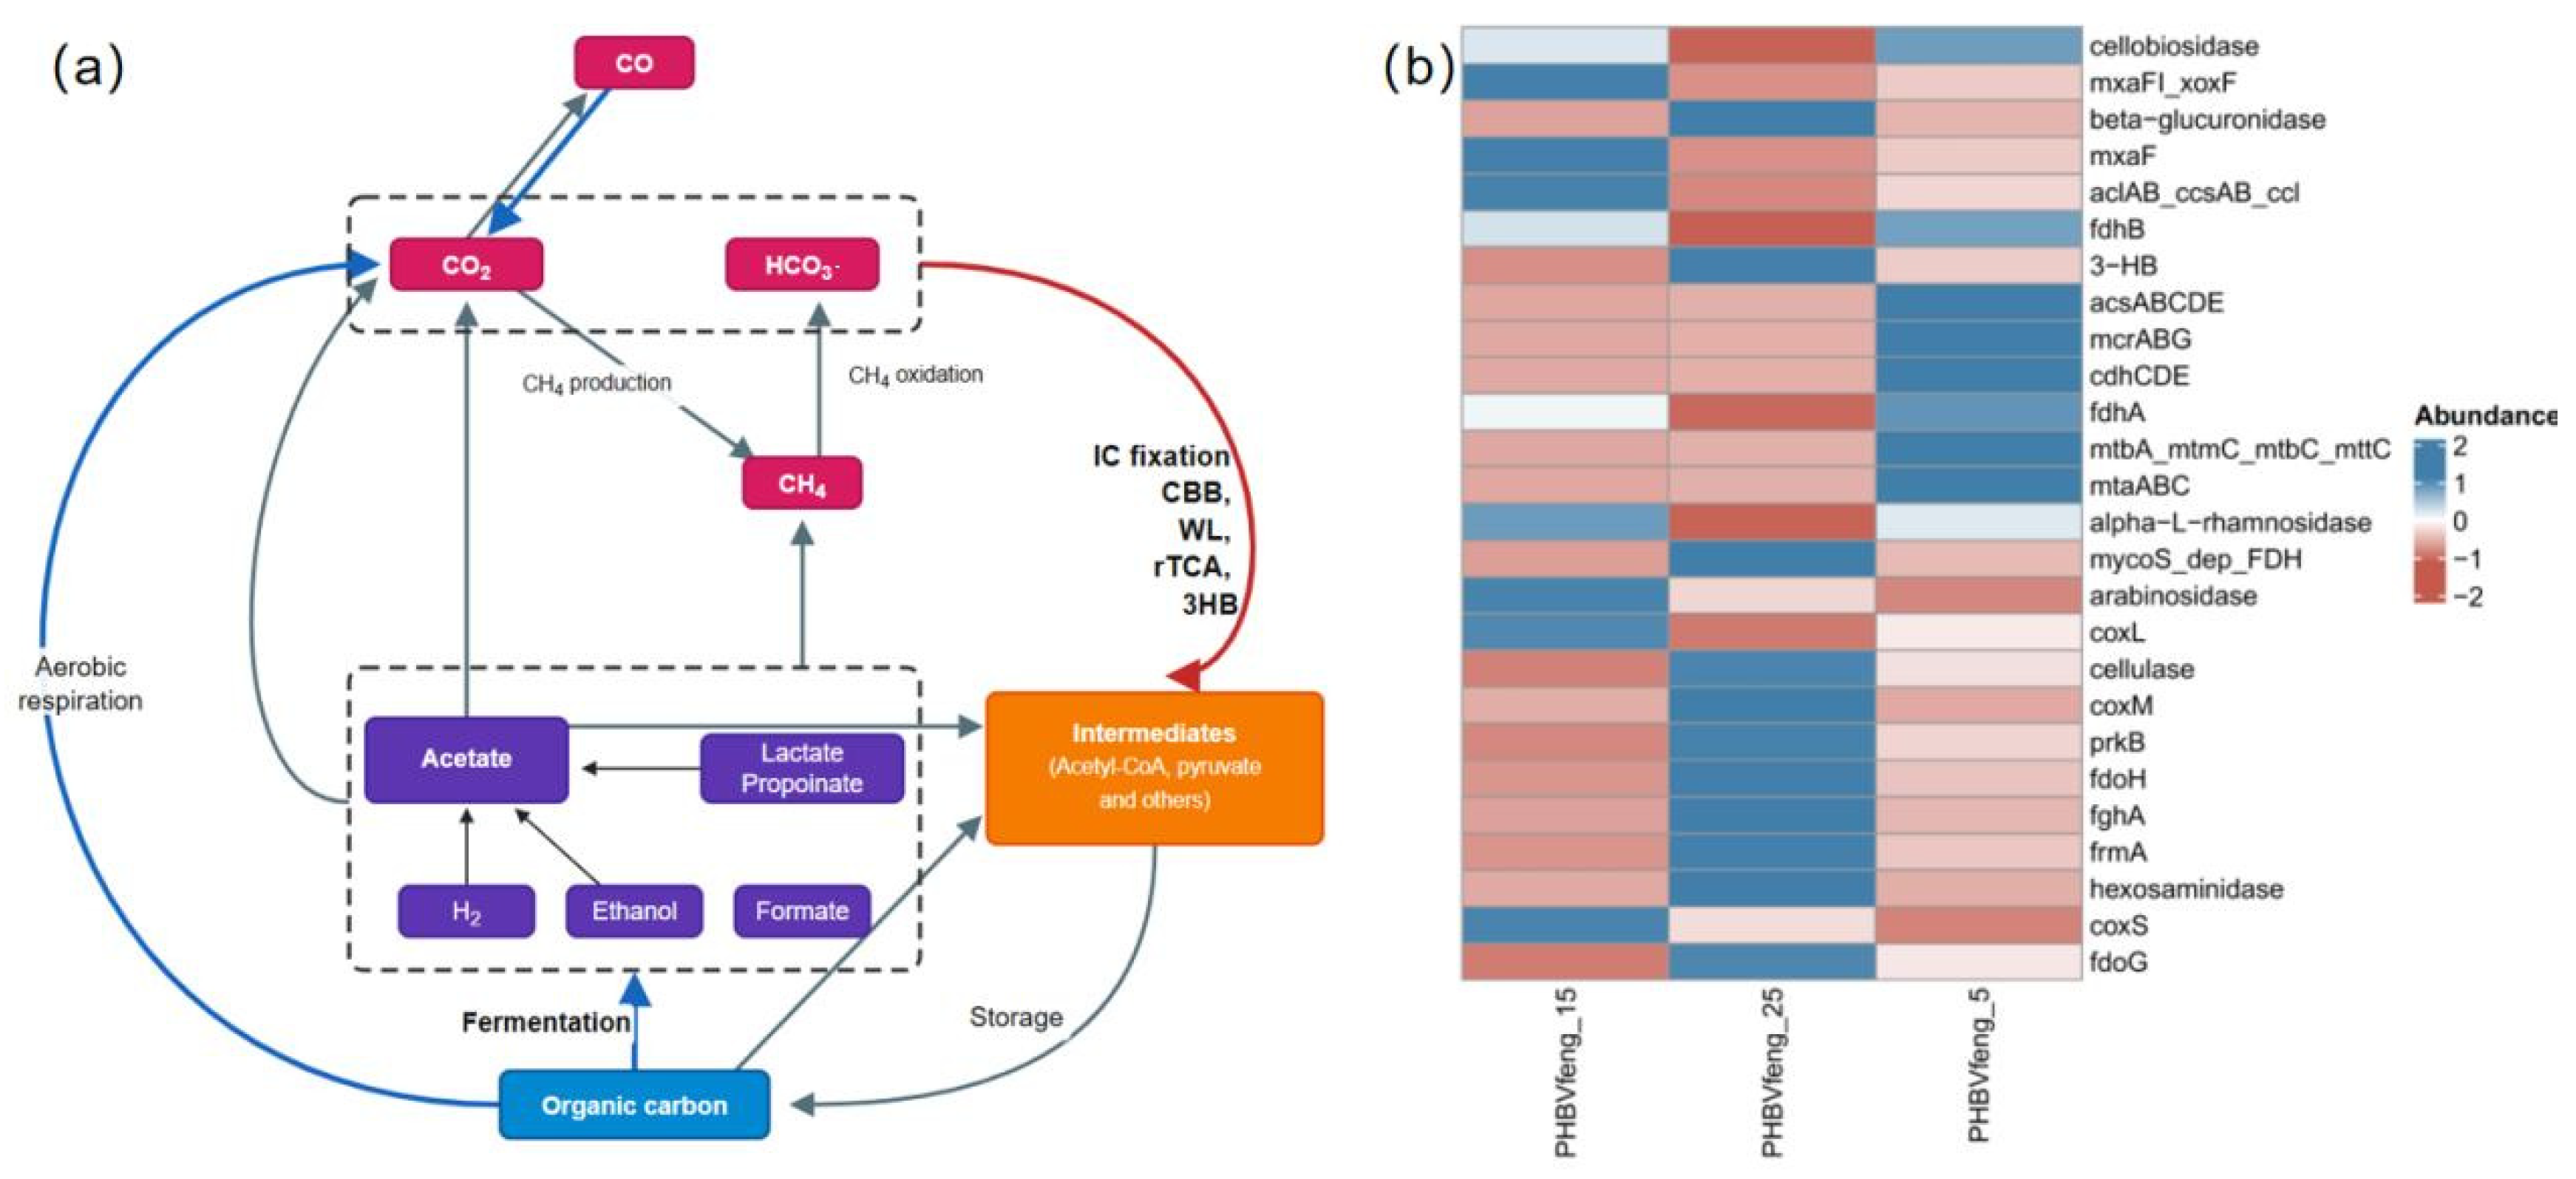
To elucidate how the microbial community senses and metabolizes PHBV-derived carbon substrates, the carbon metabolism and nitrogen cycling functional gene profiles were analyzed. The extracellular hydrolysis and intracellular transformation of solid-phase carbon sources are the key prerequisites driving the subsequent heterotrophic denitrification process [13]. The results from the carbon metabolism network diagram (Figure 7a) and the heatmap of gene abundance for enzymes involved in carbon metabolism (Figure 7b) show that environmental temperature plays a decisive role in the activation of core carbon metabolism pathways.
Figure 7.
Microbial community analysis of the biofilms on PHBV under different temperatures. (a) Relative abundance of microbial communities at the genus level. (b) Hierarchical clustering heatmap of the dominant bacterial genera. In panel (a), the dashed boxes group specific types of carbon pools: the upper box represents the inorganic carbon pool, and the lower box represents fermentation products.
At the optimal temperature of 25 °C, genes encoding key enzymes involved in the degradation of macromolecular carbohydrates exhibited significantly high expression levels (dark blue regions in Figure 7b). These include cellulase genes responsible for initial chain cleavage and hexosaminidase. In contrast, the acetyl-CoA synthase clusters (acsABCDE and cdhCDE), which play a leading role in short-chain fatty acid assimilation, exhibited higher expression at 5 °C. This counter-intuitive upregulation at low temperature likely reflects a compensatory metabolic strategy of the microbial community to maximize the capture and utilization of limited carbon intermediates under cold stress, as noted in previous studies of microbial adaptation to temperature fluctuations. Meanwhile, the robust depolymerization at 25 °C ensures that the biofilm community is highly active in capturing and assimilating small-molecule fatty acids produced by hydrolysis [29], continuously converting them into cellular energy (while also producing electron donors such as NADH required for denitrification) [30], thereby driving the highly efficient downstream denitrification cascade [28,31].
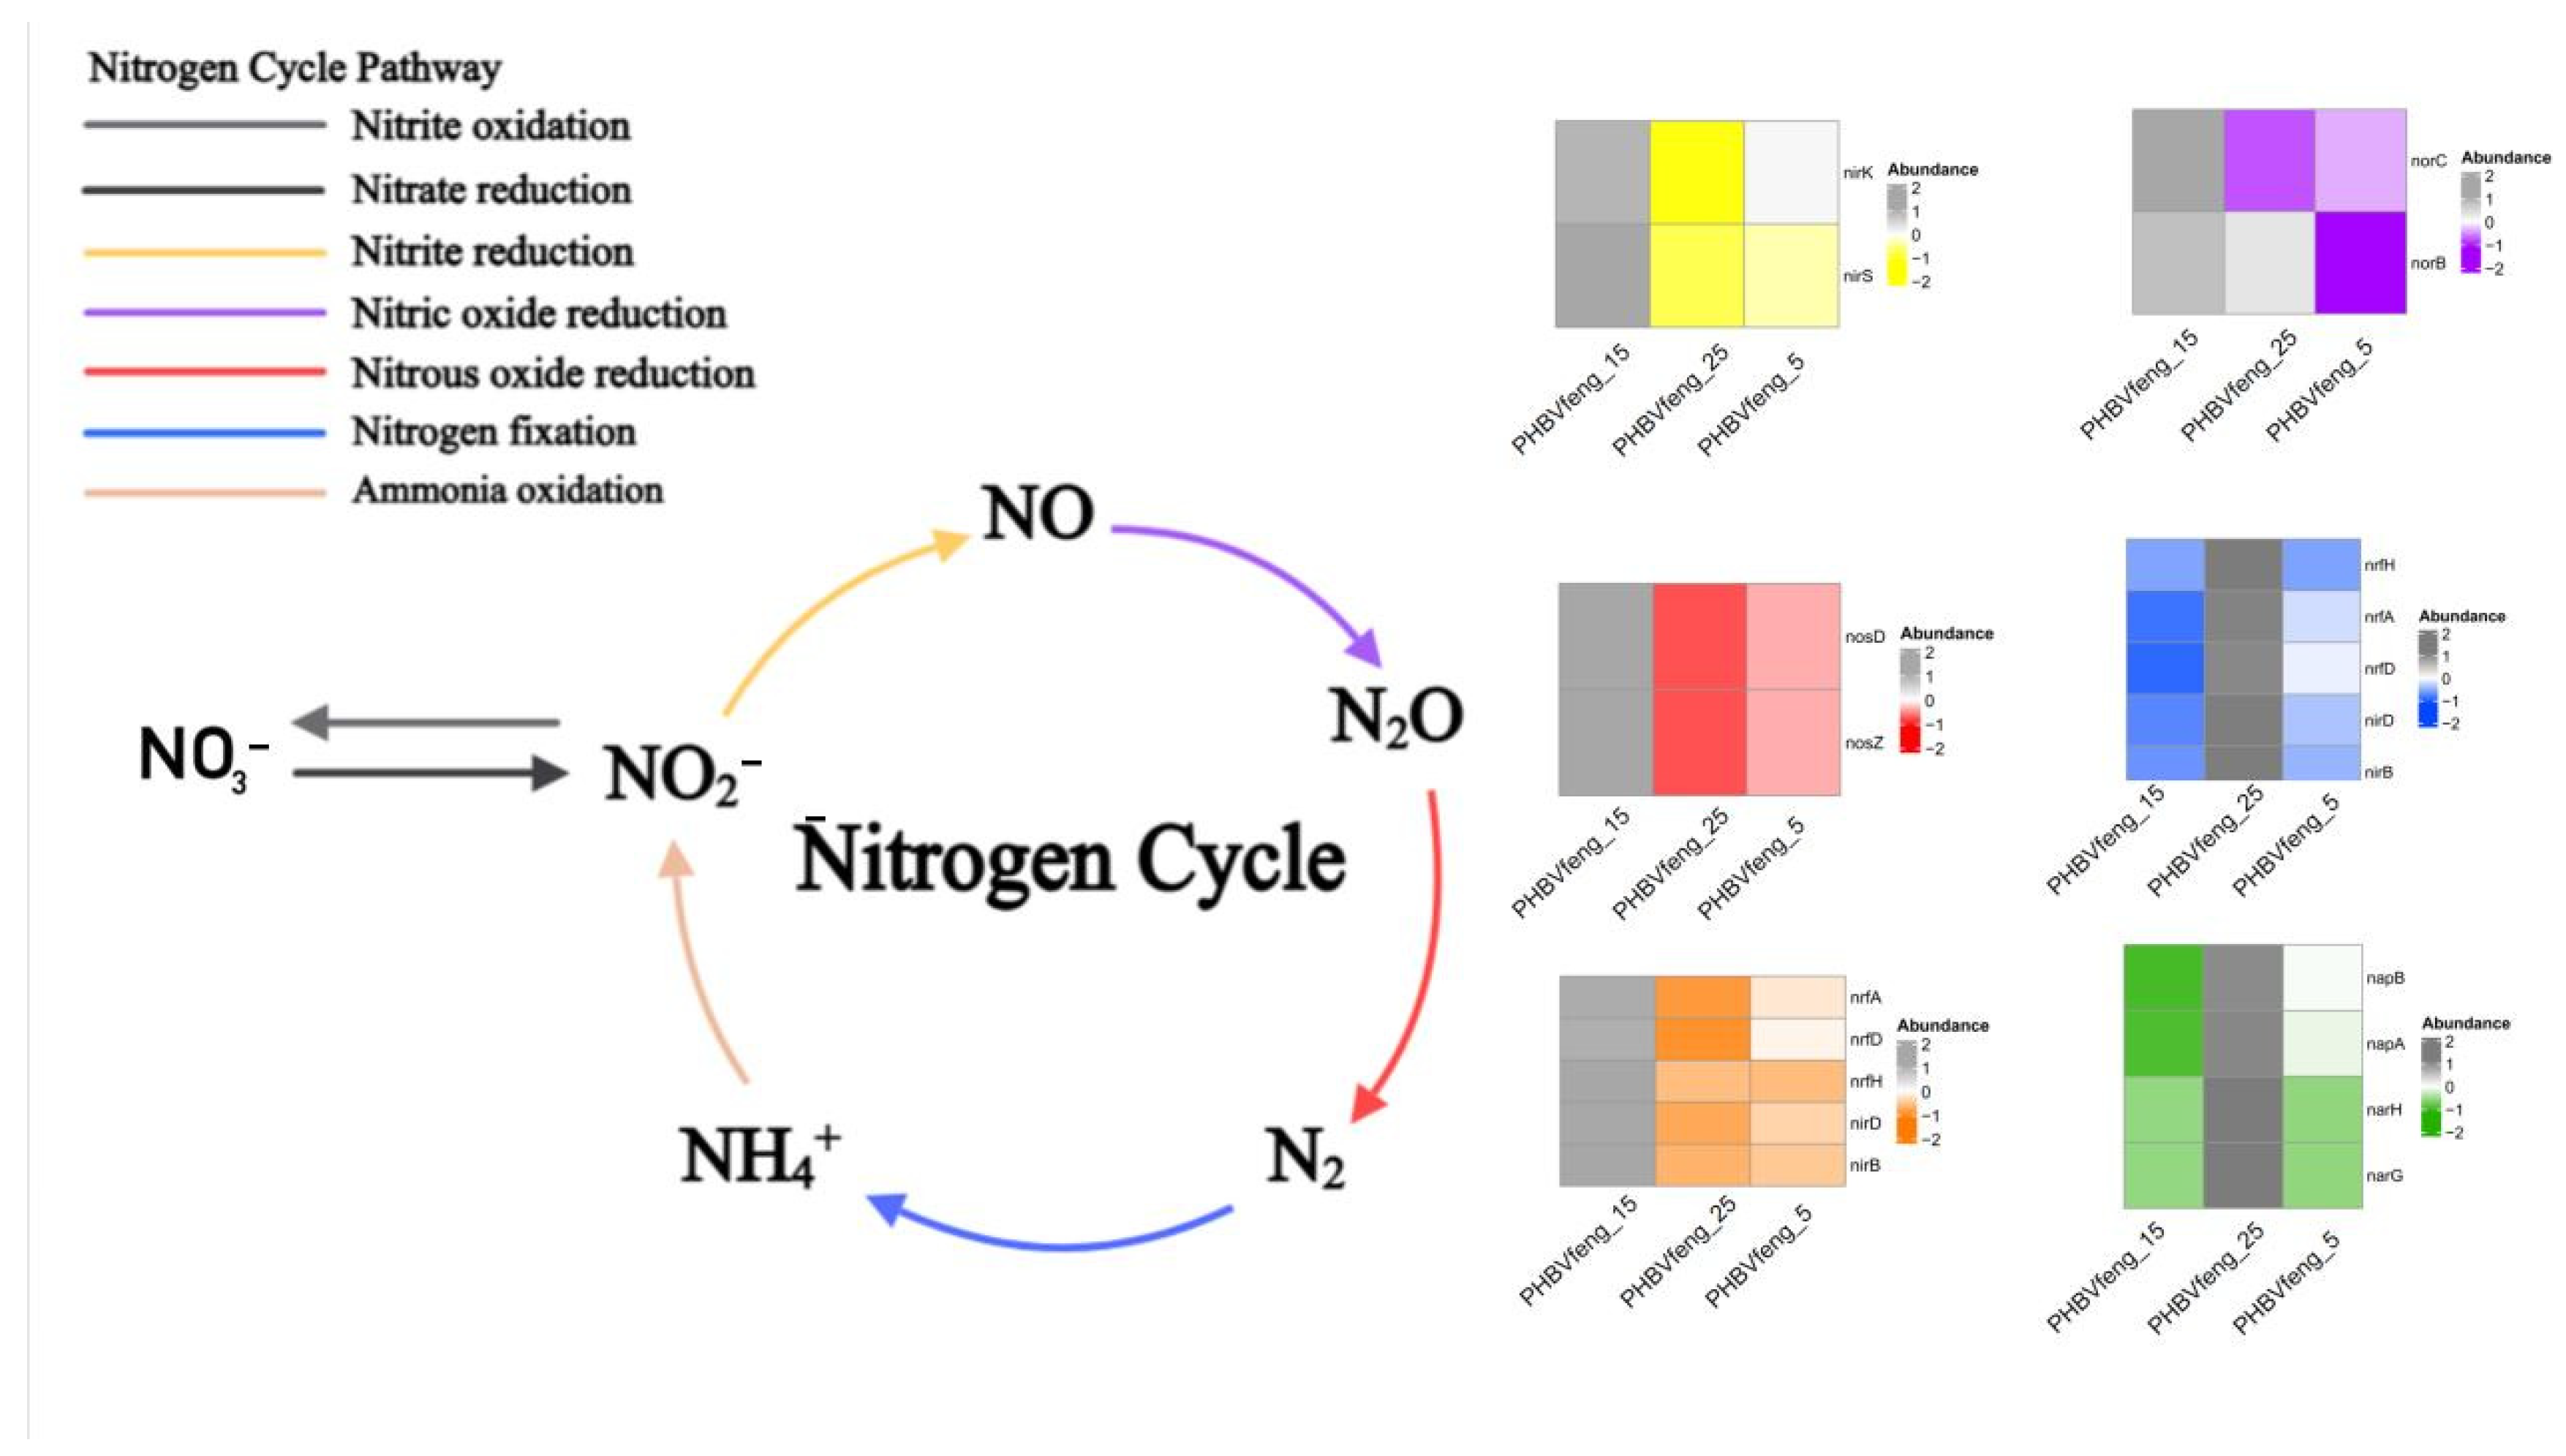
At 25 °C, the microbial community exhibits a strong ability to degrade organic carbon backbones and convert them into small molecules, enabling efficient depolymerization of PHBV and its conversion, via metabolic networks (Figure 7a), into highly bioavailable intermediate metabolites such as acetate. In contrast, under low-temperature stress at 5 °C and 15 °C, the relative abundances of the aforementioned key depolymerase and carbon metabolism genes declined. This may be because low temperatures severely inhibit the kinetics of bioenzymatic degradation of solid-phase polymers [23]; this leads to a shortage of available electron donors within the system, which in turn limits the macroscopic denitrification efficiency [13]. High-quality electron donors (such as acetate) generated by upstream carbon metabolism networks directly drive the smooth operation of downstream nitrogen cycle cascade reactions [10]. The results of the heatmap of key genes in the nitrogen cycle pathway and their relative abundances (Figure 8) show that the nitrate reductase genes (narGHI, napAB), which reduce nitrate to nitrite, and the nitrite reductase genes (nirS, nirK), which catalyze the subsequent core rate-limiting step, exhibit high transcription levels at 25 °C. This may be related to the level-dependent regulation of denitrase gene cluster transcription by electron donors [28]. Crucially, the genes encoding nitrous oxide reductases (nosZ, nosD), which catalyze the reduction of N2O to its final product, N2, were stably expressed at 25 °C (Figure 8). This observation indicates that the PHBV-associated community possesses the functional potential for complete denitrification through to N2 [32]. However, the presence of nosZ/nosD transcripts reflects genetic capacity rather than demonstrated N2O mitigation. Therefore, while the DOM released by PHBV may contribute to the reduction of NO3− and exhibits genetic potential for mitigating N2O accumulation, direct measurement of N2O emission fluxes is required to confirm this environmental safety hypothesis. Nevertheless, the stable expression of nos genes provides a theoretical rationale for the engineering application of PHBV as a solid-phase carbon source and identifies N2O flux monitoring as a priority for subsequent field-scale studies.
Figure 8.
Nitrogen transformation pathways and the abundance heatmap of functional genes involved in the nitrogen cycle driven by PHBV.
Several limitations of this study should be acknowledged. The carbon release experiments were conducted in distilled water without sterilizing the polymer granules or the reaction system; therefore, the observed DOC release represents a combined contribution from abiotic hydrolysis and incidental microbial degradation by indigenous surface-attached microorganisms or airborne contaminants, rather than pure abiotic hydrolysis. Furthermore, the environmental safety implications of PHBV-derived DOM, particularly regarding N2O emissions, were inferred from functional gene abundance rather than direct flux measurements; future studies should integrate direct N2O flux monitoring, ecotoxicological assessments of PHBV leachates, and comparative investigations across multiple BP materials to validate the broader applicability of the mechanistic framework established here.
4. Conclusions
This study systematically elucidated the carbon release characteristics of BPs in aquatic environments and the mechanisms by which they influence the microecological processes of heterotrophic denitrification. Quantitative kinetic analysis indicated that microbially synthesized PHBV exhibited the highest bioavailability as a carbon source, mediating a maximum denitrification rate of 0.72 mg/(g·h). FT-IR and UV-Vis spectroscopy confirmed that pH and photoaging accelerated surface microhydrolysis, but the PHBV polymer backbone remained highly stable, continuously releasing highly reactive aliphatic oligomers with low aromaticity. Furthermore, 16S rRNA gene amplicon sequencing results indicate that under optimal conditions at 25 °C, the abundance of genes involved in macromolecular depolymerization (cellulase, hexosaminidase) was significantly higher than at lower temperatures, inducing the directed enrichment of the core denitrifying genus Thauera and enhancing denitrification efficiency. The nitrous oxide reductase genes (nosZ, nosD) exhibited strongly temperature-dependent expression, with upregulation at 25 °C indicating the genetic potential for complete denitrification through to N2. This study provides robust scientific evidence supporting both the advanced purification of low-C/N effluent and the in situ resource utilization of BPs.
Supplementary Materials
The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/w18172165/s1, Table S1: Physicochemical specifications of the six biodegradable plastics used in this study.
Author Contributions
Conceptualization, L.D. and L.K.; methodology, S.L. and X.Z.; formal analysis, S.L. and X.Z.; writing—original draft preparation, J.H. and X.Z.; writing—review and editing, J.H. and L.K.; visualization, J.H. and L.K.; supervision, L.D.; funding acquisition, Y.C. and L.D. All authors have read and agreed to the published version of the manuscript.
Funding
This study was jointly supported by National Natural Science Foundation of China (32501503), the Changsha Natural Science Foundation (kq2502035), and the science and technology innovation Program of Hunan Province (2025AQ2005, 2025AQ2003).
Data Availability Statement
The original contributions presented in this study are included in the article/Supplementary Materials. Further inquiries can be directed to the corresponding authors.
Acknowledgments
We also thank the School of Ecology and Environment, Central South University of Forestry and Technology for providing the experimental platform, as well as the anonymous reviewers for their constructive comments and suggestions.
Conflicts of Interest
The authors declare no conflict of interest.
References
- Filiciotto, L.; Rothenberg, G. Biodegradable Plastics: Standards, Policies, and Impacts. ChemSusChem 2021, 14, 56–72. [Google Scholar] [CrossRef] [Scilit]
- Teixeira, S.C.; De Oliveira, T.V.; Fortes-Da-Silva, P.; Raymundo-Pereira, P.A.; Ribeiro, A.R.C.; Batista, L.F.; Gomes, N.O.; Stringheta, P.C.; De Fátima Ferreira Soares, N. Investigation of the Influence of Plasticizers on the Biodegradability of Cellulose Acetate. J. Appl. Polym. Sci. 2023, 140, e54316. [Google Scholar] [CrossRef] [Scilit]
- Lu, J.; Dong, Z.-H.; Zhou, J.-Q.; Li, M.; Zhang, Z.-Z.; Zhang, Y.; Jin, R.-C. Biodegradable Microplastics in Municipal Wastewater and Sludge Treatment Processes: A Review on Occurrence, Fate, and Effects. ACS EST Water 2024, 4, 8–19. [Google Scholar] [CrossRef] [Scilit]
- Niu, S.; Gao, S.; Zhang, K.; Li, Z.; Wang, G.; Li, H.; Xia, Y.; Tian, J.; Yu, E.; Xie, J.; et al. Effects of Hydraulic Retention Time and Influent Nitrate Concentration on Solid-Phase Denitrification System Using Wheat Husk as Carbon Source. PeerJ 2023, 11, e15756. [Google Scholar] [CrossRef] [Scilit]
- Haider, T.P.; Völker, C.; Kramm, J.; Landfester, K.; Wurm, F.R. Plastics of the Future? The Impact of Biodegradable Polymers on the Environment and on Society. Angew. Chem. Int. Ed. 2019, 58, 50–62. [Google Scholar] [CrossRef] [Scilit]
- Zhang, S.; Chang, X.; Wu, F.; Lu, Y.; An, S.; Zhou, Y.; Feng, M.; Du, Y. Alternation Magnitudes of Organic Matter Composition Determines Priming Effect of Biodegradable Microplastics on Lake Carbon Emission. Water Res. 2026, 297, 125713. [Google Scholar] [CrossRef] [Scilit]
- Xia, L.; Li, X.; Fan, W.; Wang, J. Denitrification Performance and Microbial Community of Bioreactor Packed with PHBV/PLA/Rice Hulls Composite. Sci. Total Environ. 2022, 803, 150033. [Google Scholar] [CrossRef] [Scilit]
- Xiong, R.; Yu, X.; Zhang, Y.; Peng, Z.; Yu, L.; Cheng, L.; Li, T. Comparison of Agricultural Wastes and Synthetic Macromolecules as Solid Carbon Source in Treating Low Carbon Nitrogen Wastewater. Sci. Total Environ. 2020, 739, 139885. [Google Scholar] [CrossRef] [Scilit]
- Lucas, N.; Bienaime, C.; Belloy, C.; Queneudec, M.; Silvestre, F.; Nava-Saucedo, J.-E. Polymer Biodegradation: Mechanisms and Estimation Techniques—A Review. Chemosphere 2008, 73, 429–442. [Google Scholar] [CrossRef] [Scilit]
- Feng, Y.; Wang, L.; Yin, Z.; Cui, Z.; Qu, K.; Wang, D.; Wang, Z.; Zhu, S.; Cui, H. Comparative Investigation on Heterotrophic Denitrification Driven by Different Biodegradable Polymers for Nitrate Removal in Mariculture Wastewater: Organic Carbon Release, Denitrification Performance, and Microbial Community. Front. Microbiol. 2023, 14, 1141362. [Google Scholar] [CrossRef] [Scilit]
- Gewert, B.; Plassmann, M.M.; MacLeod, M. Pathways for Degradation of Plastic Polymers Floating in the Marine Environment. Environ. Sci. Process. Impacts 2015, 17, 1513–1521. [Google Scholar] [CrossRef] [Scilit]
- Wei, Q.; Zhang, J.; Luo, F.; Shi, D.; Liu, Y.; Liu, S.; Zhang, Q.; Sun, W.; Yuan, J.; Fan, H.; et al. Molecular Mechanisms through Which Different Carbon Sources Affect Denitrification by Thauera Linaloolentis: Electron Generation, Transfer, and Competition. Environ. Int. 2022, 170, 107598. [Google Scholar] [CrossRef] [Scilit]
- Luo, F.; Zhang, J.; Wei, Q.; Jiang, Z.; Jiang, D.; Liu, S.; Xia, Z.; Zhang, J.; Qi, L.; Wang, H.; et al. Insights into the Relationship between Denitrification and Organic Carbon Release of Solid-Phase Denitrification Systems: Mechanism and Microbial Characteristics. Bioresour. Technol. 2022, 364, 128044. [Google Scholar] [CrossRef] [Scilit]
- Qiu, Y.-Y.; Gong, X.; Zhang, L.; Zhou, S.; Li, G.; Jiang, F. Achieving a Novel Polysulfide-Involved Sulfur-Based Autotrophic DenitrificationProcess for High-Rate Nitrogen Removal in Elemental Sulfur-Packed Bed Reactors. ACS EST Eng. 2022, 2, 1504–1513. [Google Scholar] [CrossRef] [Scilit]
- Jendrossek, D.; Handrick, R. Microbial Degradation of Polyhydroxyalkanoates. Annu. Rev. Microbiol. 2002, 56, 403–432. [Google Scholar] [CrossRef] [Scilit]
- Wang, J.; Chu, L. Biological Nitrate Removal from Water and Wastewater by Solid-Phase Denitrification Process. Biotechnol. Adv. 2016, 34, 1103–1112. [Google Scholar] [CrossRef] [Scilit]
- Yin, S.; Liu, R.; Shao, Y.; Zhu, J. Mechanistic Insights into Carbon Release and Denitrification in Sandwich-Structured Hydrogel Composites for Low C/N Wastewater Denitrification. Chem. Eng. Sci. 2026, 330, 123941. [Google Scholar] [CrossRef] [Scilit]
- Yu, W.; Zheng, T.; Guo, B.; Tao, Y.; Liu, L.; Yan, N.; Zheng, X. Coupling of Polyhydroxybutyrate and Zero-Valent Iron for Enhanced Treatment of Nitrate Pollution within the Permeable Reactive Barrier and Its Downgradient Aquifer. Water Res. 2024, 250, 121060. [Google Scholar] [CrossRef] [Scilit]
- Chen, Z.; Zuo, Q.; Liu, C.; Li, L.; Deliz Quiñones, K.Y.; He, Q. Insights into Solid Phase Denitrification in Wastewater Tertiary Treatment: The Role of Solid Carbon Source in Carbon Biodegradation and Heterotrophic Denitrification. Bioresour. Technol. 2023, 376, 128838. [Google Scholar] [CrossRef] [Scilit]
- Wang, J.; Sun, Y.; Khunjar, W.; Pace, G.; McGrath, M.; Chitrakar, S.; Taylor, R.L.; Carroll, J.R.; Zhang, X.; Wang, Z.-W. Mechanistic Understanding of the Performance Difference between Methanol- and Glycerol-Fed Partial Denitrification Anammox in Tertiary Moving Bed Biofilm Reactors Treating Real Secondary Effluent. Water Res. 2025, 271, 122893. [Google Scholar] [CrossRef] [Scilit]
- Huang, W.; Jiang, G.; Xie, L.; Chen, X.; Zhang, R.; Fan, X. Effect of Oxygen-Containing Functional Groups on the Micromechanical Behavior of Biodegradable Plastics and Their Formation of Microplastics during Aging. J. Hazard. Mater. 2024, 463, 132911. [Google Scholar] [CrossRef] [Scilit]
- Brdlík, P.; Borůvka, M.; Běhálek, L.; Lenfeld, P. The Influence of Additives and Environment on Biodegradation of PHBV Biocomposites. Polymers 2022, 14, 838. [Google Scholar] [CrossRef] [Scilit]
- Xu, Z.; Dai, X.; Chai, X. Biological Denitrification Using PHBV Polymer as Solid Carbon Source and Biofilm Carrier. Biochem. Eng. J. 2019, 146, 186–193. [Google Scholar] [CrossRef] [Scilit]
- Li, P.; Hur, J. Utilization of UV-Vis Spectroscopy and Related Data Analyses for Dissolved Organic Matter (DOM) Studies: A Review. Crit. Rev. Environ. Sci. Technol. 2017, 47, 131–154. [Google Scholar] [CrossRef] [Scilit]
- Liu, Y.; Chen, F.; He, Y.; Wang, Y.; Zhu, T.; Tong, Y.; Zhao, Y.; Ni, B.-J.; Liu, Y. Evaluation of Nitrous Oxide Reduction in Solid Carbon Source-Driven Counter-Diffusional Biofilm Denitrification System. Water Res. X 2025, 27, 100306. [Google Scholar] [CrossRef] [Scilit]
- Yang, Z.; Lou, Y.; Pan, H.; Wang, H.; Yang, Q.; Zhuge, Y.; Hu, J. Improved Denitrification Performance of Polybutylene Succinate/Corncob Composite Carbon Source by Proper Pretreatment: Performance, Functional Genes and Microbial Community Structure. Polymers 2023, 15, 801. [Google Scholar] [CrossRef] [Scilit]
- Tec-Campos, D.; Tibocha-Bonilla, J.D.; Jiang, C.; Passi, A.; Thiruppathy, D.; Zuñiga, C.; Posadas, C.; Zepeda, A.; Zengler, K. A Genome-Scale Metabolic Model for the Denitrifying Bacterium Thauera sp. MZ1T Accurately Predicts Degradation of Pollutants and Production of Polymers. PLoS Comput. Biol. 2025, 21, e1012736. [Google Scholar] [CrossRef] [Scilit]
- Oba, K.; Suenaga, T.; Kuroiwa, M.; Riya, S.; Terada, A. Exploring the Functions of Efficient Canonical Denitrifying Bacteria as N2O Sinks: Implications from 15N Tracer and Transcriptome Analyses. Environ. Sci. Technol. 2022, 56, 11694–11706. [Google Scholar] [CrossRef] [Scilit]
- Zhang, X.; Song, X.; Cheng, X.; Huang, Z.; Dong, D.; Li, X. Enhanced Denitrification of Biodegradable Polymers Using Bacillus Pumilus in Aerobic Denitrification Bioreactors: Performance and Mechanism. Bioresour. Technol. 2024, 394, 130240. [Google Scholar] [CrossRef] [Scilit]
- Si, G.-C.; Wei, D.; He, C.; Shi, Q.; Sheng, G.-P. Revealing Dissolved Organic Nitrogen Transformation and Microbial Evolution at Microscale in a Solid Carbon Source-Coordinated Simultaneous Partial Nitrification, Anammox, and Denitrification Bioreactor. ACS EST Eng. 2022, 2, 2066–2075. [Google Scholar] [CrossRef] [Scilit]
- Adam, P.S.; Borrel, G.; Gribaldo, S. Evolutionary History of Carbon Monoxide Dehydrogenase/Acetyl-CoA Synthase, One of the Oldest Enzymatic Complexes. Proc. Natl. Acad. Sci. USA 2018, 115, E1166–E1173. [Google Scholar] [CrossRef] [Scilit]
- Pan, Y.; Ni, B.-J.; Yuan, Z. Modeling Electron Competition among Nitrogen Oxides Reduction and N2O Accumulation in Denitrification. Environ. Sci. Technol. 2013, 47, 11083–11091. [Google Scholar] [CrossRef] [Scilit]
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.