Article

Internal Cycling Influences Nutrient Changes Leading to Altered Nutrient Limitation in Eutrophic Lake


1
School of Energy and Environment Science, Yunnan Normal University, Kunming 650500, China
2
Faculty of Geography, Yunnan Normal University, Kunming 650500, China
3
GIS Technology Engineering Research Centre for West China Resources and Environment, Ministry Education, Yunnan Normal University, Kunming 650500, China
*
Authors to whom correspondence should be addressed.
Water 2025, 17(17), 2604; https://doi.org/10.3390/w17172604
Submission received: 25 July 2025 / Revised: 23 August 2025 / Accepted: 1 September 2025 / Published: 3 September 2025
(This article belongs to the Section Biodiversity and Functionality of Aquatic Ecosystems)

Abstract

Lake eutrophication is governed by persistent anthropogenic nutrient inputs, primarily nitrogen (N), phosphorus (P) and cryptic internal nutrient cycling processes that sustain bioavailable nutrient pools. While the impact of external nutrient loads on lake eutrophication has been extensively studied, the role of internal nutrient cycling in lake ecosystems remains underexplored. In this study, the hierarchical bootstrap generalized linear model (HBGLM) to long-term summer water quality data (1999–2020) from Lake Dianchi, China, to explore the relative importance of nitrogen (N), phosphorus (P), as well as the limitations of N and P on the growth of phytoplankton. The results revealed that from 1999 to 2020, the Chla and TP concentrations decreased by 49% and 78%, respectively, and that internal nutrient cycling significantly influenced changes in nutrient concentrations, reflecting the relationships among N, P, and chlorophyll a (Chla). Particularly in 2007, 2013, and 2017, the long-term trends of the TN:TP ratio, an indicator of potential nutrient limitation in the lake, were consistent with changes in the distributions of the average slopes of TN and TP across different periods, indicating that these years primarily exhibited patterns of colimitation by N and P or P limitation, indirectly confirming that Lake Dianchi will transition from N and P colimitation to being limited primarily by P. This study reveals that N is typically the primary limiting element, while P is a key element promoting water eutrophication. To further validate improvements to existing eutrophication mitigation models, conducting carefully de-signed experiments at different scales is recommended.

1. Introduction

Lake eutrophication is among the major water environmental problems worldwide [1,2,3], with direct ecological consequences, including the occurrence of harmful algal blooms (HABs) [4], frequent algal blooms [5], fish death, decreased dissolved oxygen in water bodies, and the disappearance of submerged plants [6,7]. Since the 1970s, management has long emphasized that phosphorus (P) is the key limiting factor in controlling eutrophication [8,9], but in recent years, recent studies based on large-scale datasets have demonstrated the role of nitrogen (N) limitation or the colimitation of N and P in shallow lakes, especially in shallow eutrophic lakes [10,11,12,13], and under certain levels of nutrient enrichment, the limiting factor may undergo a transformation from being P limited to being colimited [14,15,16,17].
Nutrient concentrations and the related ratio of total nitrogen (TN):total phosphorus (TP) are not only affected by external nutrient loading but also strongly regulated by the endogenous nutrient cycle. This cycle manifests as the release of N and P from lake bottom sediments through processes such as denitrification, resuspension, and mineralization into the water body, thereby affecting the nutrient acquisition of phytoplankton [1,18,19]. During periods of heavy external loading and high phytoplankton biomass, P tends to accumulate in sediment and be retained in lakes [20,21], whereas the retention or release of N is more complicated and is affected mainly by the denitrification rate. After a sufficient reduction in external nutrient loading, the accumulated P can be released into the overlying lake water, which sustains high P concentrations [22]. In contrast, the response of N seems faster due to loss through denitrification [23,24], which leads to less accumulation of N than P in sediment [25]. Compared to P, the removal rate of N is faster and is controlled by the denitrification rate. It has a more complex response mechanism [23,24,26]. Particularly in shallow lakes, factors such as lake depth, hydraulic retention time (HRT), and sediment structure significantly influence the accumulation and release processes of N and P [27,28].
Lake Dianchi is a typical shallow semi-enclosed lake in southwestern China. It has been affected by urbanization and agricultural emissions for a long time. The external load has significantly decreased [29], but the concentration of P in the lake remains high, indicating that the internal load may be an important source for maintaining eutrophication [30]. This is different from the situation of other semi-enclosed lakes (such as those with different exchange cycles) [31]. The water retention time of Lake Dianchi is long [32], and nutrients are prone to accumulation, resulting in different inputs of external nutrients in the internal circulation process [30]. As a result, with decreasing external load, the internal circulation response of the lake can be relatively long [1]. In this context, it is difficult to achieve water quality improvement merely by controlling external inputs. There is an urgent need to identify the nutrient limitation mechanisms driven by internal cycles (i.e., sediment release, nitrification and denitrification) and further clarify the key nutrient elements that should be prioritized for control when managing algal biomass. Currently, most studies on nutrient limitation changes are static or short-term experiments, and long-term dynamic research on the N:P limitation relationship is lacking. In this paper, on the basis of the monitoring data of Lake Dianchi from 1999 to 2020, hierarchical bootstrapping for generalized linear models (HBGLM) was adopted, and a large amount of long-term observation data collected over 22 years was used to study the dynamic changes in chlorophyll a (Chla) and nutrient levels during the 22-year period, the relative influence of TN and TP on Chla in different time windows was quantified, and the changing trends of nutrient limitation patterns were identified. The HBGLM method, which combines generalized linear models with bootstrapping, effectively retains the temporal structure and spatial heterogeneity of the lake system. It is suitable for shallow water lake environments with nonlinear ecological responses and complex changes in nutrient status. This method has been widely applied in lake ecological metrology in recent years and is advantageous for handling long time series, hierarchical structures, and model uncertainties [17,33]. This approach can be used to elucidate the dynamic mechanism underlying the effects of nitrogen and phosphorus on algal biomass. A major question has emerged from attempts at lake restoration: what impact does the reduction in nutrients leading to changes in the internal circulation process have on the nutrient restriction pattern of algal growth, reflected in the nutrient relationship among N, P and Chla, and which element should be prioritized for control, namely, nitrogen, phosphorus, or both? To study nitrogen and phosphorus limitation issues in shallow lakes, it is necessary to dynamically analyse the limiting mechanisms under different nutrient conditions, especially the response mechanisms when endogenous loading is dominant, and to formulate targeted water quality management and pollution control strategies [34]. This is highly important for the ecological governance of Lake Dianchi and other shallow lakes.

2. Materials and Methods

2.1. Study Area and Data Sources

Lake Dianchi (102°29′–103°01′ E, 24°29′–25°28′ N) is located in the middle of the Yunnan–Kweichow Plateau and is oriented north to south (Figure 1). Lake Dianchi has 35 tributaries flowing into it, and there is only one outlet in the Haikou area. The lake has an elevation of approximately 1886 m, a catchment area of approximately 2920 km2, an average water depth of approximately 5 m, and a maximum depth of up to 10.7 metres. It is a typical shallow semi-enclosed lake [35]. Lake Dianchi is located downstream of Kunming city and has a subtropical humid monsoon climate. The annual average temperature, precipitation and evaporation are 14.7 °C, 938.77 mm and 1409.4 mm, respectively [36]. The average hydraulic retention time (HRT) is 3.5 years, and the water exchange capacity of the lake is limited, making it prone to nutrient enrichment. Over the past 40 years, it has experienced urbanization, industrial development and intensified agricultural activities, which have caused eutrophication. The bottom sediment of the inner lake (Caohai) area of Lake Dianchi is black and rich in humus and contains semidecomposed plant debris with an iron-like odour. This type of muddy bottom sediment is rich in organic matter, which is one of the manifestations of lake eutrophication. Sandy loam bottom sediment is commonly found in the outer lake area. Gravelly sandy soil is distributed along the shoreline, with relatively large particles and good permeability.
Lake Dianchi has eight monitoring stations, which are located at Huiwanzhong, Guanyinshanxi, Guanyinshanzhong, Guanyinshandong, Dianchinan, Haikouxi, Luojiaying and Baiyukou (Figure 1 and Table 1). These stations are distributed primarily across different directions in the outer lake area of Lake Dianchi, effectively covering the main regions of the outer lake. The degradation of water quality stems from multiple factors, such as population growth and urban expansion.
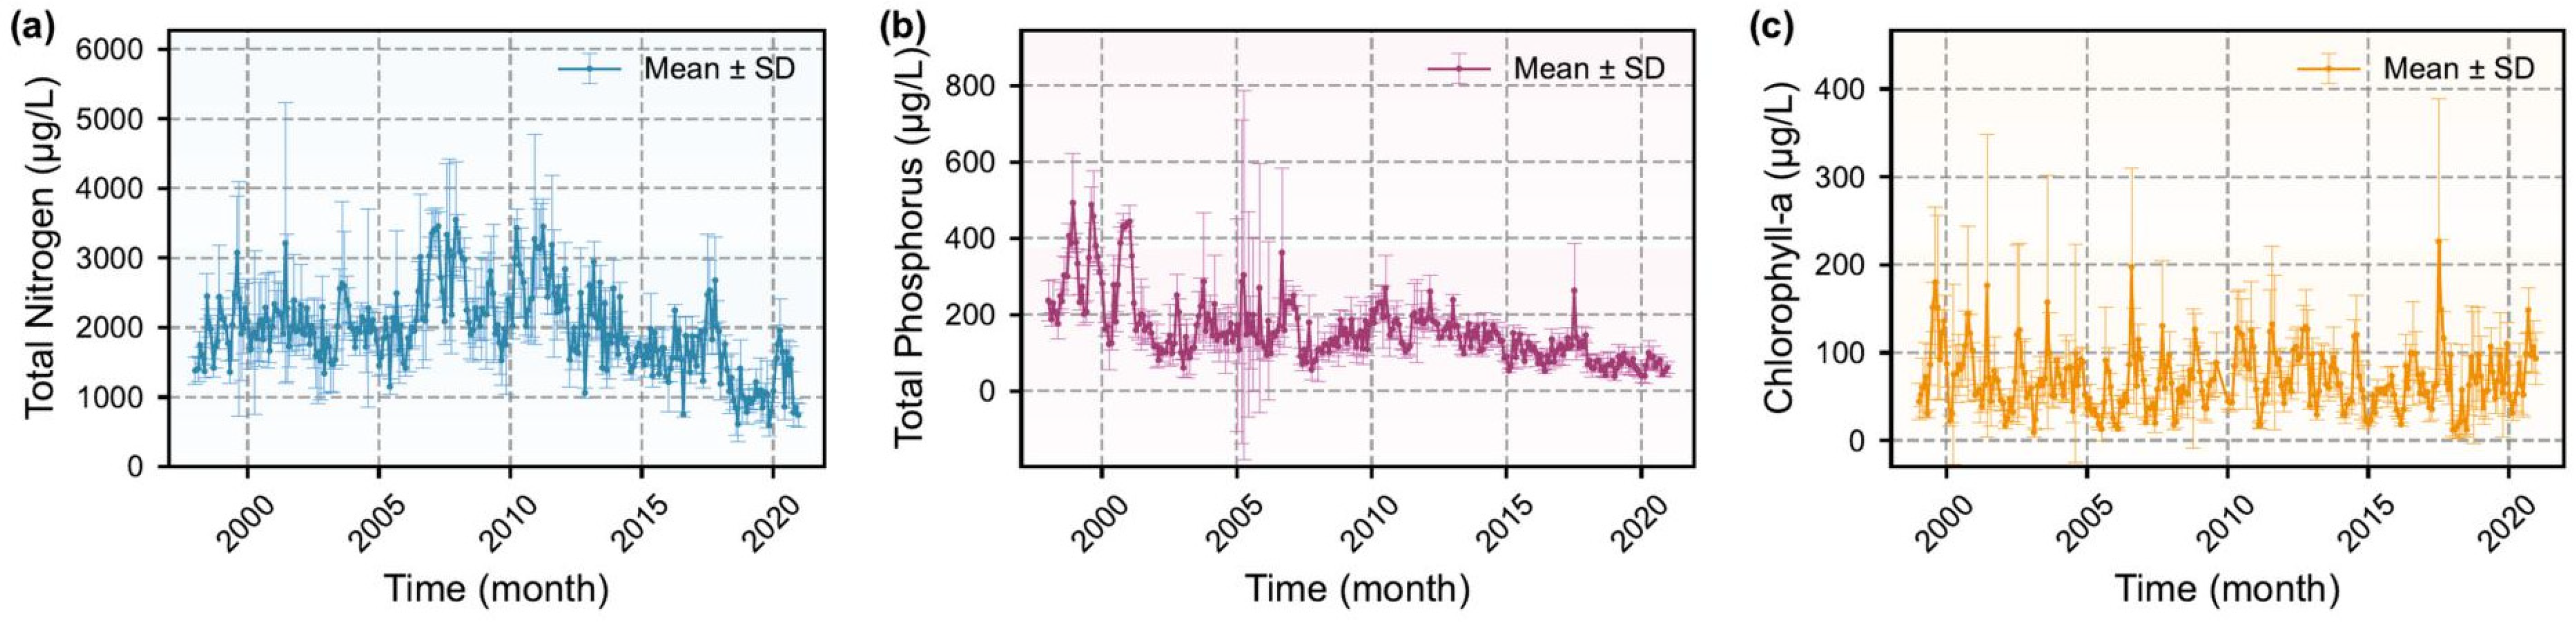
TN and TP concentrations exhibit significant spatial heterogeneity, with pollution patterns decreasing from north to south. During high-temperature periods, algal blooms are prone to occur in the Caohai area and northeastern nearshore regions. The shoreline zone, which is the primary area where pollutants converge and is heavily influenced by anthropogenic activities, has more monitoring stations established. The lake centre zone, with stable and uniform water quality, has only one station set up for background value monitoring and comparative analysis. Although spatial heterogeneity in nutrient concentrations exists, with higher values typically observed in the northern and northeastern nearshore zones, the overall variability among the eight monitoring stations is relatively small, as demonstrated in Figure 2. This figure shows temporal variations in monthly average concentrations of TN (a), TP (b), and Chla (c).

2.2. Environmental Data Collection and Processing

Long-term water quality data for Lake Dianchi (1999–2020) were obtained from the Kunming Environmental Monitoring Center (KEMC). Monitoring was conducted at eight fixed sampling stations (Figure 1) on a monthly basis (one sampling campaign per month). Water samples were collected at each sampling point from the surface layer at a depth of 0.5 m below the water surface. TN was determined using the alkaline potassium persulfate digestion ultraviolet spectrophotometric method (GB/T 11894-1989) [37], and TP was determined using the ammonium molybdate spectrophotometric method (GB/T 11893-1989). The Chla concentration was determined by spectrophotometry after extraction with 90% hot ethanol.
These data provide a basis for selecting and verifying the model established in this study. Long-term observations, including TP, TN, and Chla levels, were used in this study. Seasons were defined as follows: spring (March–May), summer (June–August), autumn (September–November), and winter (December–February) [38]. Summer is selected to capture peak internal nutrient cycling, driven by thermal stratification and sediment phosphorus release. This study focuses primarily on summer dynamic changes in N and P concentrations and Chla concentrations in water bodies and does not include data on N and P contents in sediment deposits. Currently, N and P data for Lake Dianchi sediments can be found in existing studies [37].

2.3. Statistical Data Analyses

2.3.1. Long-Term Trends in Water Quality

Temporal trends were visualized using weighted regression with bootstrapped smoothers. This function calculates smoothers from 1000 bootstraps of the original samples, followed by the calculation of density estimates for each vertical cut through the bootstrapped smoothers, which are then visualized by shade colour and intensity [38,39]. Moreover, local polynomial regression (loess) was employed to fit the trend of the data. The uncertainty interval of the trend was constructed through bootstrap sampling. Multiple pseudo data sets were generated by randomly sampling the original data. The loess trend line was fitted for each data set, and finally, the fluctuation range of the trend was determined by the statistical quantiles (2.5–97.5%). The algorithm explicitly addressed model uncertainty through ensemble learning, mitigating the problem of different or conflicting interpretations of the same data due to inconsistencies between algorithms [40]. This approach has been previously applied to ecological and environmental domains [41,42,43,44].

2.3.2. Hierarchical Bootstrap for the Generalized Linear Model Method

The hierarchical bootstrap (HBS) method was first proposed by Graeber et al. [17]. It was used to establish hierarchical bootstraps for generalized linear models (HBGLMs) that could effectively reflect the overall data structure, retain information about the lake, and explore the relative importance of nitrogen and phosphorus to Chla under different trophic states. First, the lakes were classified into three categories on the basis of their Chla concentration: low–moderate trophic (Chla ≤ 7 μg·L−1), eutrophic (7 μg·L−1 < Chla ≤ 30 μg·L−1) and hypereutrophic (Chla > 30 μg·L−1). The GLMs were established with Chla as the response variable and TN or TP as the explanatory variable. We used TN and total phosphorus (TP) as explanatory variables in the HBGLM for the following reasons: 1. TN and TP act as stoichiometric integrators of multiple chemical forms and internal–external processes, providing robust indicators of potential nutrient limitations at decadal scales [17,44,45]. 2. Long-term monthly records of fractionated nitrogen and phosphorus (e.g., DIN, SRP, DON, DOP, and PP) were not consistently available for 1999–2020; including them would substantially reduce the sample size and introduce methodological heterogeneity, whereas TN and TP have the greatest consistency in time and space and in terms of methods. 3. In shallow eutrophic lakes, TN and TP better capture the net outcome of coupled external loading and internal cycling (sediment–water exchange, denitrification, resuspension) [46,47]. To avoid collinearity and enhance interpretability, we established HBGLMs for TN and TP separately and compared the pseudo-R2, slopes, and AIC within a 10-year moving window; before modelling, all the variables were log-transformed to mitigate skewness and scale effects [33]. For Chla, a lognormal distribution was preferred; all the variables were log-transformed (natural logarithm), and the normal distribution was used as the linked distribution for the generalized linear models (GLMs). We extracted R2 (pseudo-R2 = 1 − model bias/zero bias), Akaike’s information criterion (AIC), the model slope, and the intercept of the GLMs for demonstration.
To gain a deeper understanding of the relationship between nutrients (N and P) and lake eutrophication, we further investigated the issue of nutrient limitation in lake eutrophication. This study uses Chla as a key indicator of water quality, which reflects the biomass of phytoplankton and algae in water bodies. Algal biomass is a core characteristic of lake eutrophication and is an important component of water quality assessment. Higher Chla concentrations indicate more severe eutrophication and poorer water quality [48,49]. To reveal temporal trends, the framework of HBGLMs is commonly used [33]. We used HBGLMs to explore the possible nonlinear relationships between algal biomass dynamics and nutrient concentrations. The concentration of Chla is significantly positively correlated with the actual biomass of the phytoplankton. Therefore, it is widely used in lake ecology research as a reliable substitute indicator for phytoplankton biomass and can effectively reflect dynamic changes in phytoplankton biomass [50,51]. To determine when and to what extent internal nutrient concentrations influence changes in algal biomass, in the HBGLM analyses, internal nutrient (TN and TP) concentrations were used as explanatory variables, and water quality (Chla) was used as a response variable to determine the relative effects of nutrient (TN and TP) concentrations on water quality in Lake Dianchi from 1999 to 2020. The annual average was estimated using a 10-year simple moving window to eliminate short-term changes while retaining long-term information. The average values during this period were summarized on an annual basis, and logarithmic transformation was performed before modelling. The nonparametric bias residual bootstrap method of HBGLMs fixes the fitted values of the raw data and creates a bootstrap by adding bootstrap samples of the residuals to the fitted values to obtain a bootstrap response [17,41]. In this study, the HBGLM method was used to analyse the correlations among the three scenarios of N limitation, P limitation and N and P colimitation in the Lake Dianchi region and the influencing factors.

3. Results

3.1. Temporal Dynamics of Nutrients and TN:TP Stoichiometry in Lake Dianchi

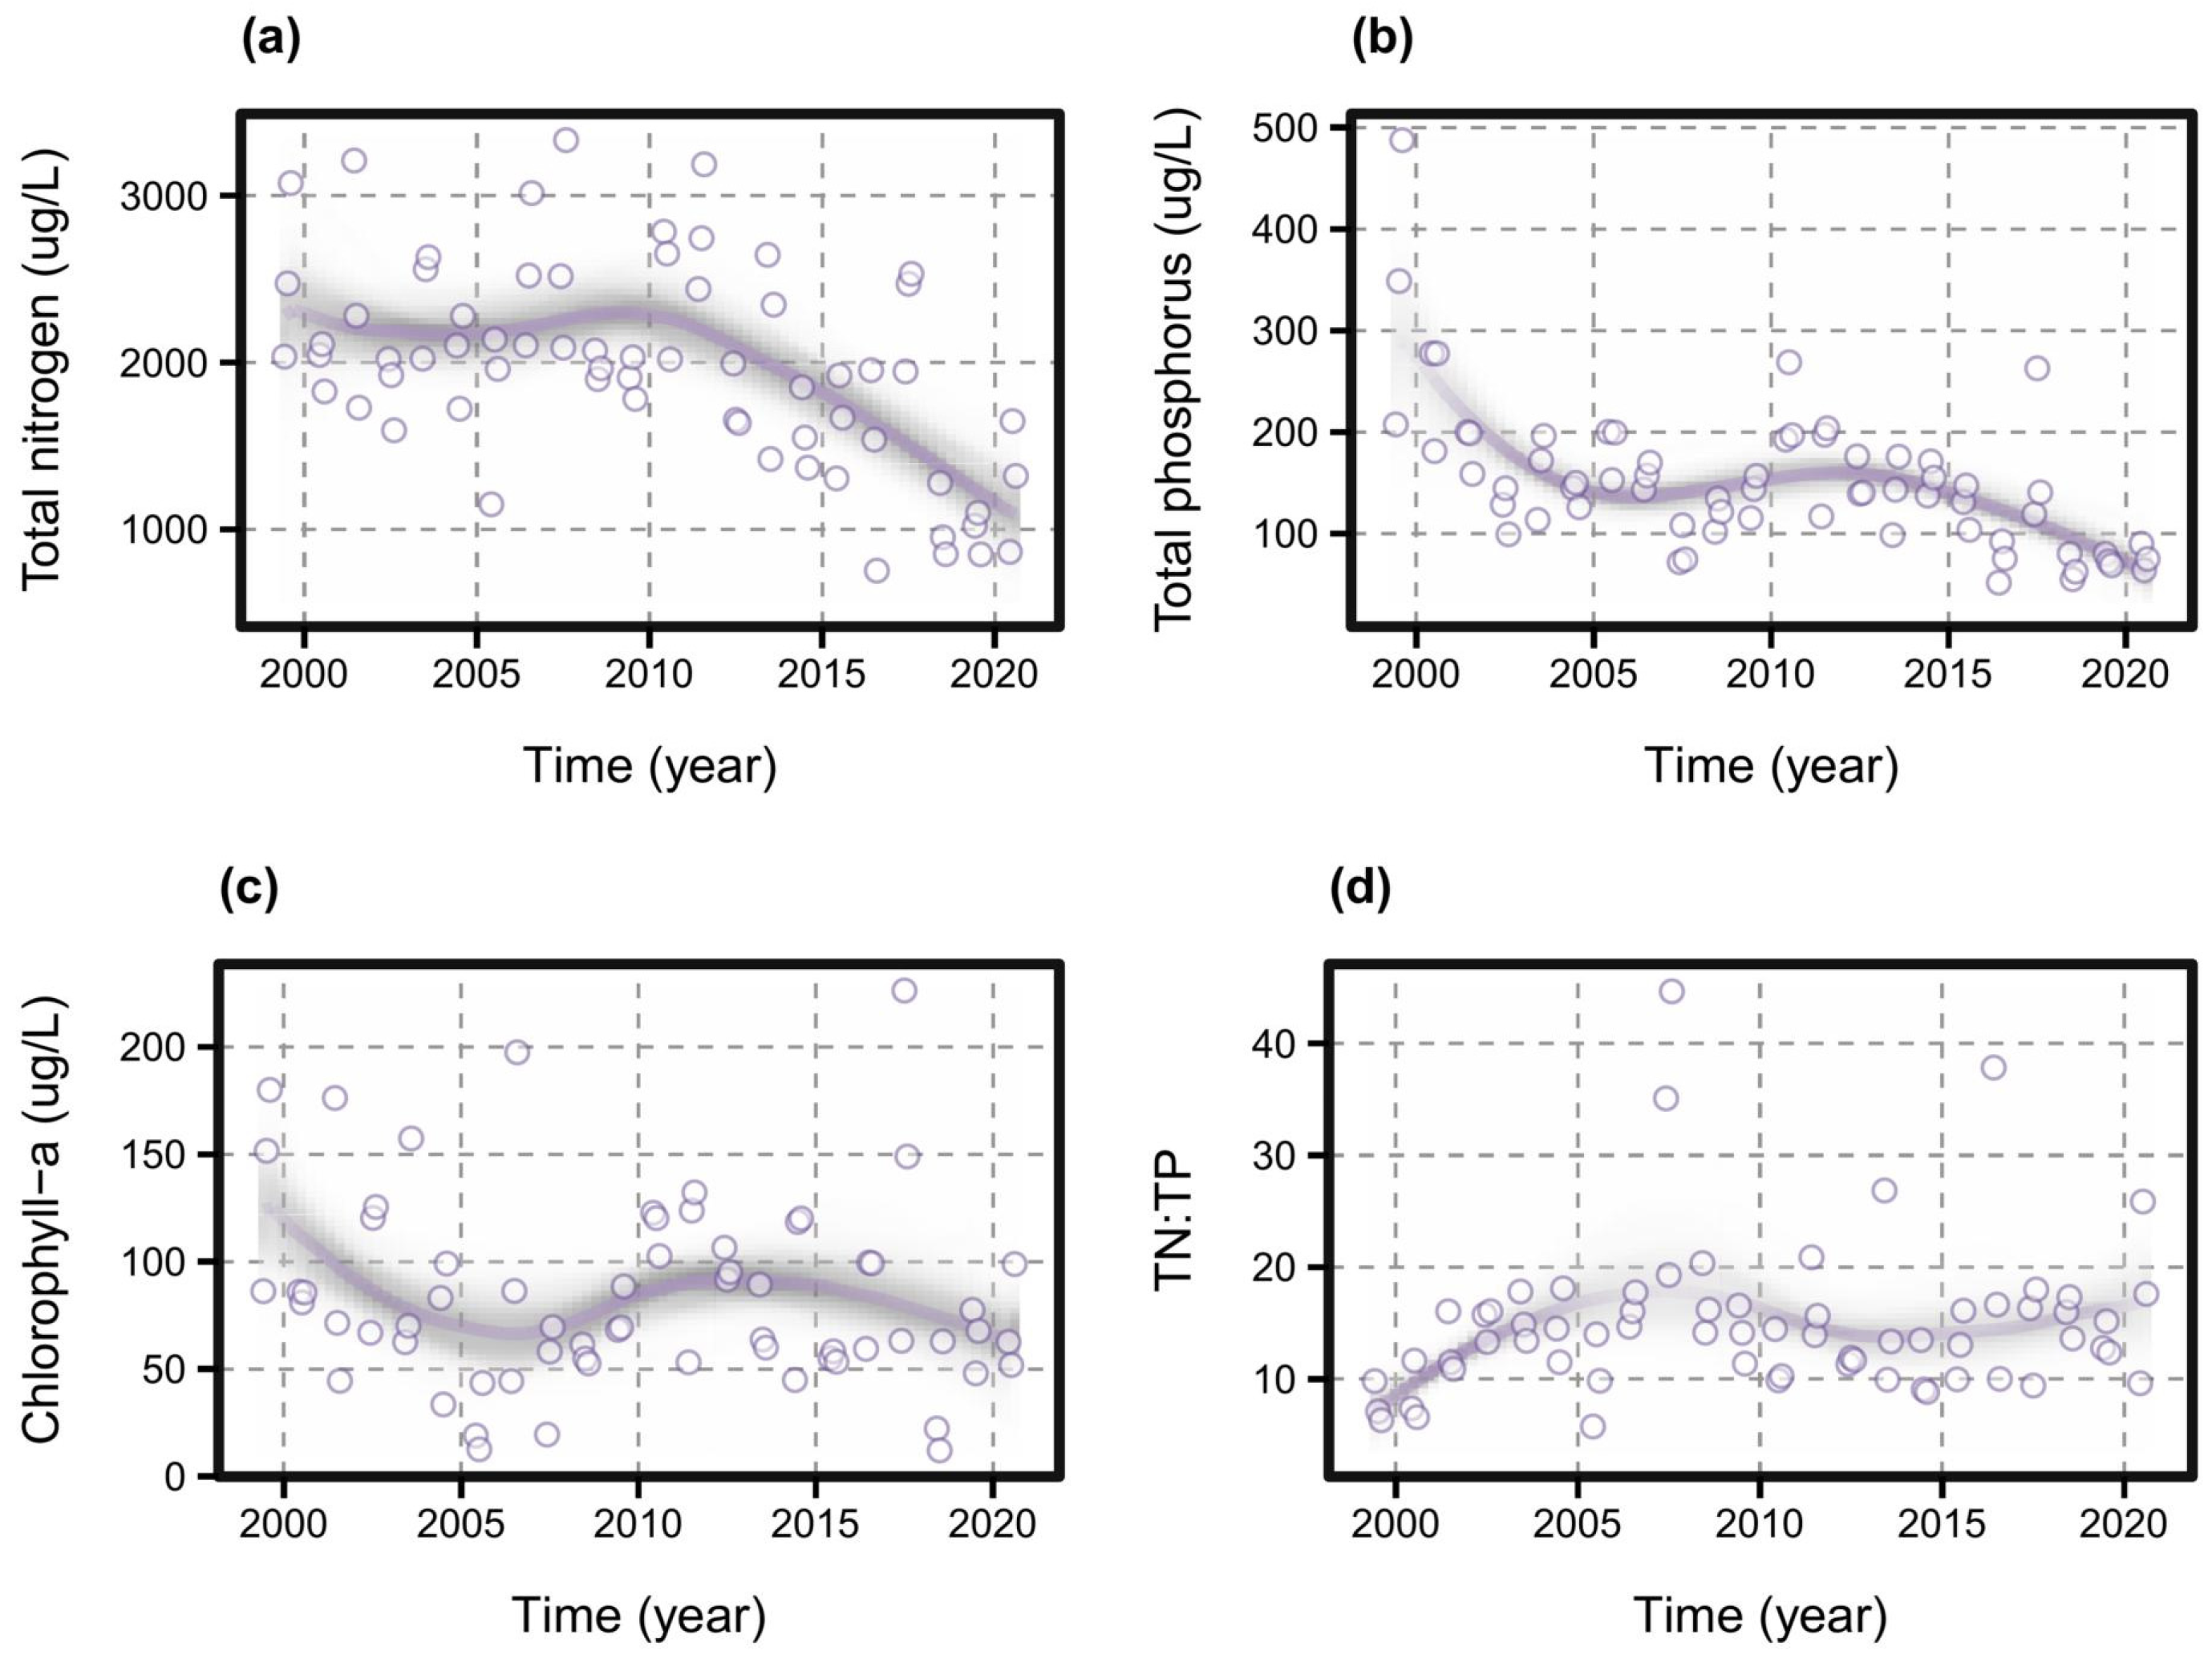
The summer TN concentration range from 1999 to 2020 was 752.5–3332.5 μg·L−1. The summer TN concentrations were relatively high before 2010, increasing from 2278.75 μg·L−1 in 1999 to 2346.25 μg·L−1 in 2009 and then significantly decreasing to 1098.25 μg·L−1 from 2009 to 2020. The overall trend of summer TN showed a slow increase followed by a significant decrease, reaching the lowest point in nearly 22 years. The average summer TN concentration from 1999 to 2020 was 1975.6 ± 515.3 μg·L−1 (Figure 3a). From 1999 to 2020, the summer TP concentration ranged from 51.63 to 487.5 μg·L−1. During the period from 1999 to 2005, the summer TP concentration tended to decrease, from 347.92 μg·L−1 in 1999 to 152.75 μg·L−1, followed by a slight increase from 2005 to 2012. From 2012 to 2020, summer TP concentrations decreased significantly from 151.88 μg·L−1 to 63.75 μg·L−1. The overall trend of the summer TP concentration initially significantly decreased (with the highest summer TP concentration occurring in approximately 1999), followed by a slight increase and then a significant decline at the inflection point from 2012 to the lowest summer TP concentration (Figure 3b). The average summer TP concentration from 1999 to 2020 was 150.7 ± 64.7 μg·L−1. The concentration range of Chla during the summer from 1999 to 2020 was 12.13–226.25 μg·L−1. The Chla concentration significantly decreased from 1999 to 2006, dropping to 67.5 μg·L−1. By approximately 2006, summer chlorophyll-a concentrations had fallen below 75 μg·L−1 and reached their lowest point. From 2006 to 2013, summer chlorophyll-a concentrations subsequently tended to increase slowly. This was followed by a gradual decline from 2013 to 2020, when the lowest point was reached. In 2013, the concentration decreased from 89.38 μg·L−1 to 63.75 μg·L−1, and by 2020, summer Chla concentrations had decreased below 60 μg·L−1, reaching the lowest point (Figure 3c). The overall trend in summer Chla concentrations significantly decreased (with Chla concentrations reaching their highest levels in nearly 22 years in 1999), followed by a slow increase and, finally, a slow decline to the lowest Chla concentrations in nearly 22 years. Similarly, summer TP concentrations also exhibited the same trend. The average summer Chla concentration from 1999 to 2020 was 83.9 ± 30.7 μg·L−1. The N:P ratio doctrine, guided by ecological stoichiometry and Liebig’s law of least limiting factors, proposes that the TN:TP ratio (by mass) can be used as an indicator of potential lake nutrient limitations. Changes in the stoichiometry of TN:TP can indicate altered nutrient limitation patterns in phytoplankton [16]. On the basis of thresholds derived from global phytoplankton stoichiometry models, nitrogen is the limiting factor when N:P < 9.0 (potential mononitrogen limitation exists); when 9 ≤ N:P < 22.6, nitrogen and phosphorus are colimiting (N + P symbiosis exists); and when N:P ≥ 22.6, phosphorus is the limiting factor (monophosphorus limitation exists) [16,51].
The range of the TN:TP ratio (by mass) in the summer from 1999 to 2020 was 5.7–44.7. From 1999 to 2007, the TN:TP ratio (by mass) tended to increase from 6.3 to 20.4. The TN:TP ratio in the summer of approximately 2007 was not less than 20. In terms of the changes in TN:TP stoichiometry, the nutrient restriction pattern of Lake Dianchi in summer gradually changed from the N imitation pattern in 1999 to the common N and P colimitation pattern. From 2007 to 2012, the summer TN:TP ratio (by mass) tended to decrease slightly, but there were significant interannual fluctuations, gradually decreasing from 18.7 to 13.6. Lake Dianchi is still characterized by both nitrogen and phosphorus limitations. From 2012 to 2020, the summer TN:TP ratio (by mass) slightly increased, increasing from 13.3 to 17.6. However, the level was still lower than the peak values before and after 2007; overall, it evolved towards the P limitation threshold, but most years within the study period remained within the common N and P colimitation pattern (Figure 3d). Lake Dianchi is predicted to gradually shift to a P-limited nutrient model in the future.
In aquatic ecosystems, the TN:TP ratio is an important indicator of nutrient balance. Both excessively high and low TN:TP ratios have significant effects on aquatic ecosystems [37,52].

3.2. Temporal Dynamics of N and P on Chla

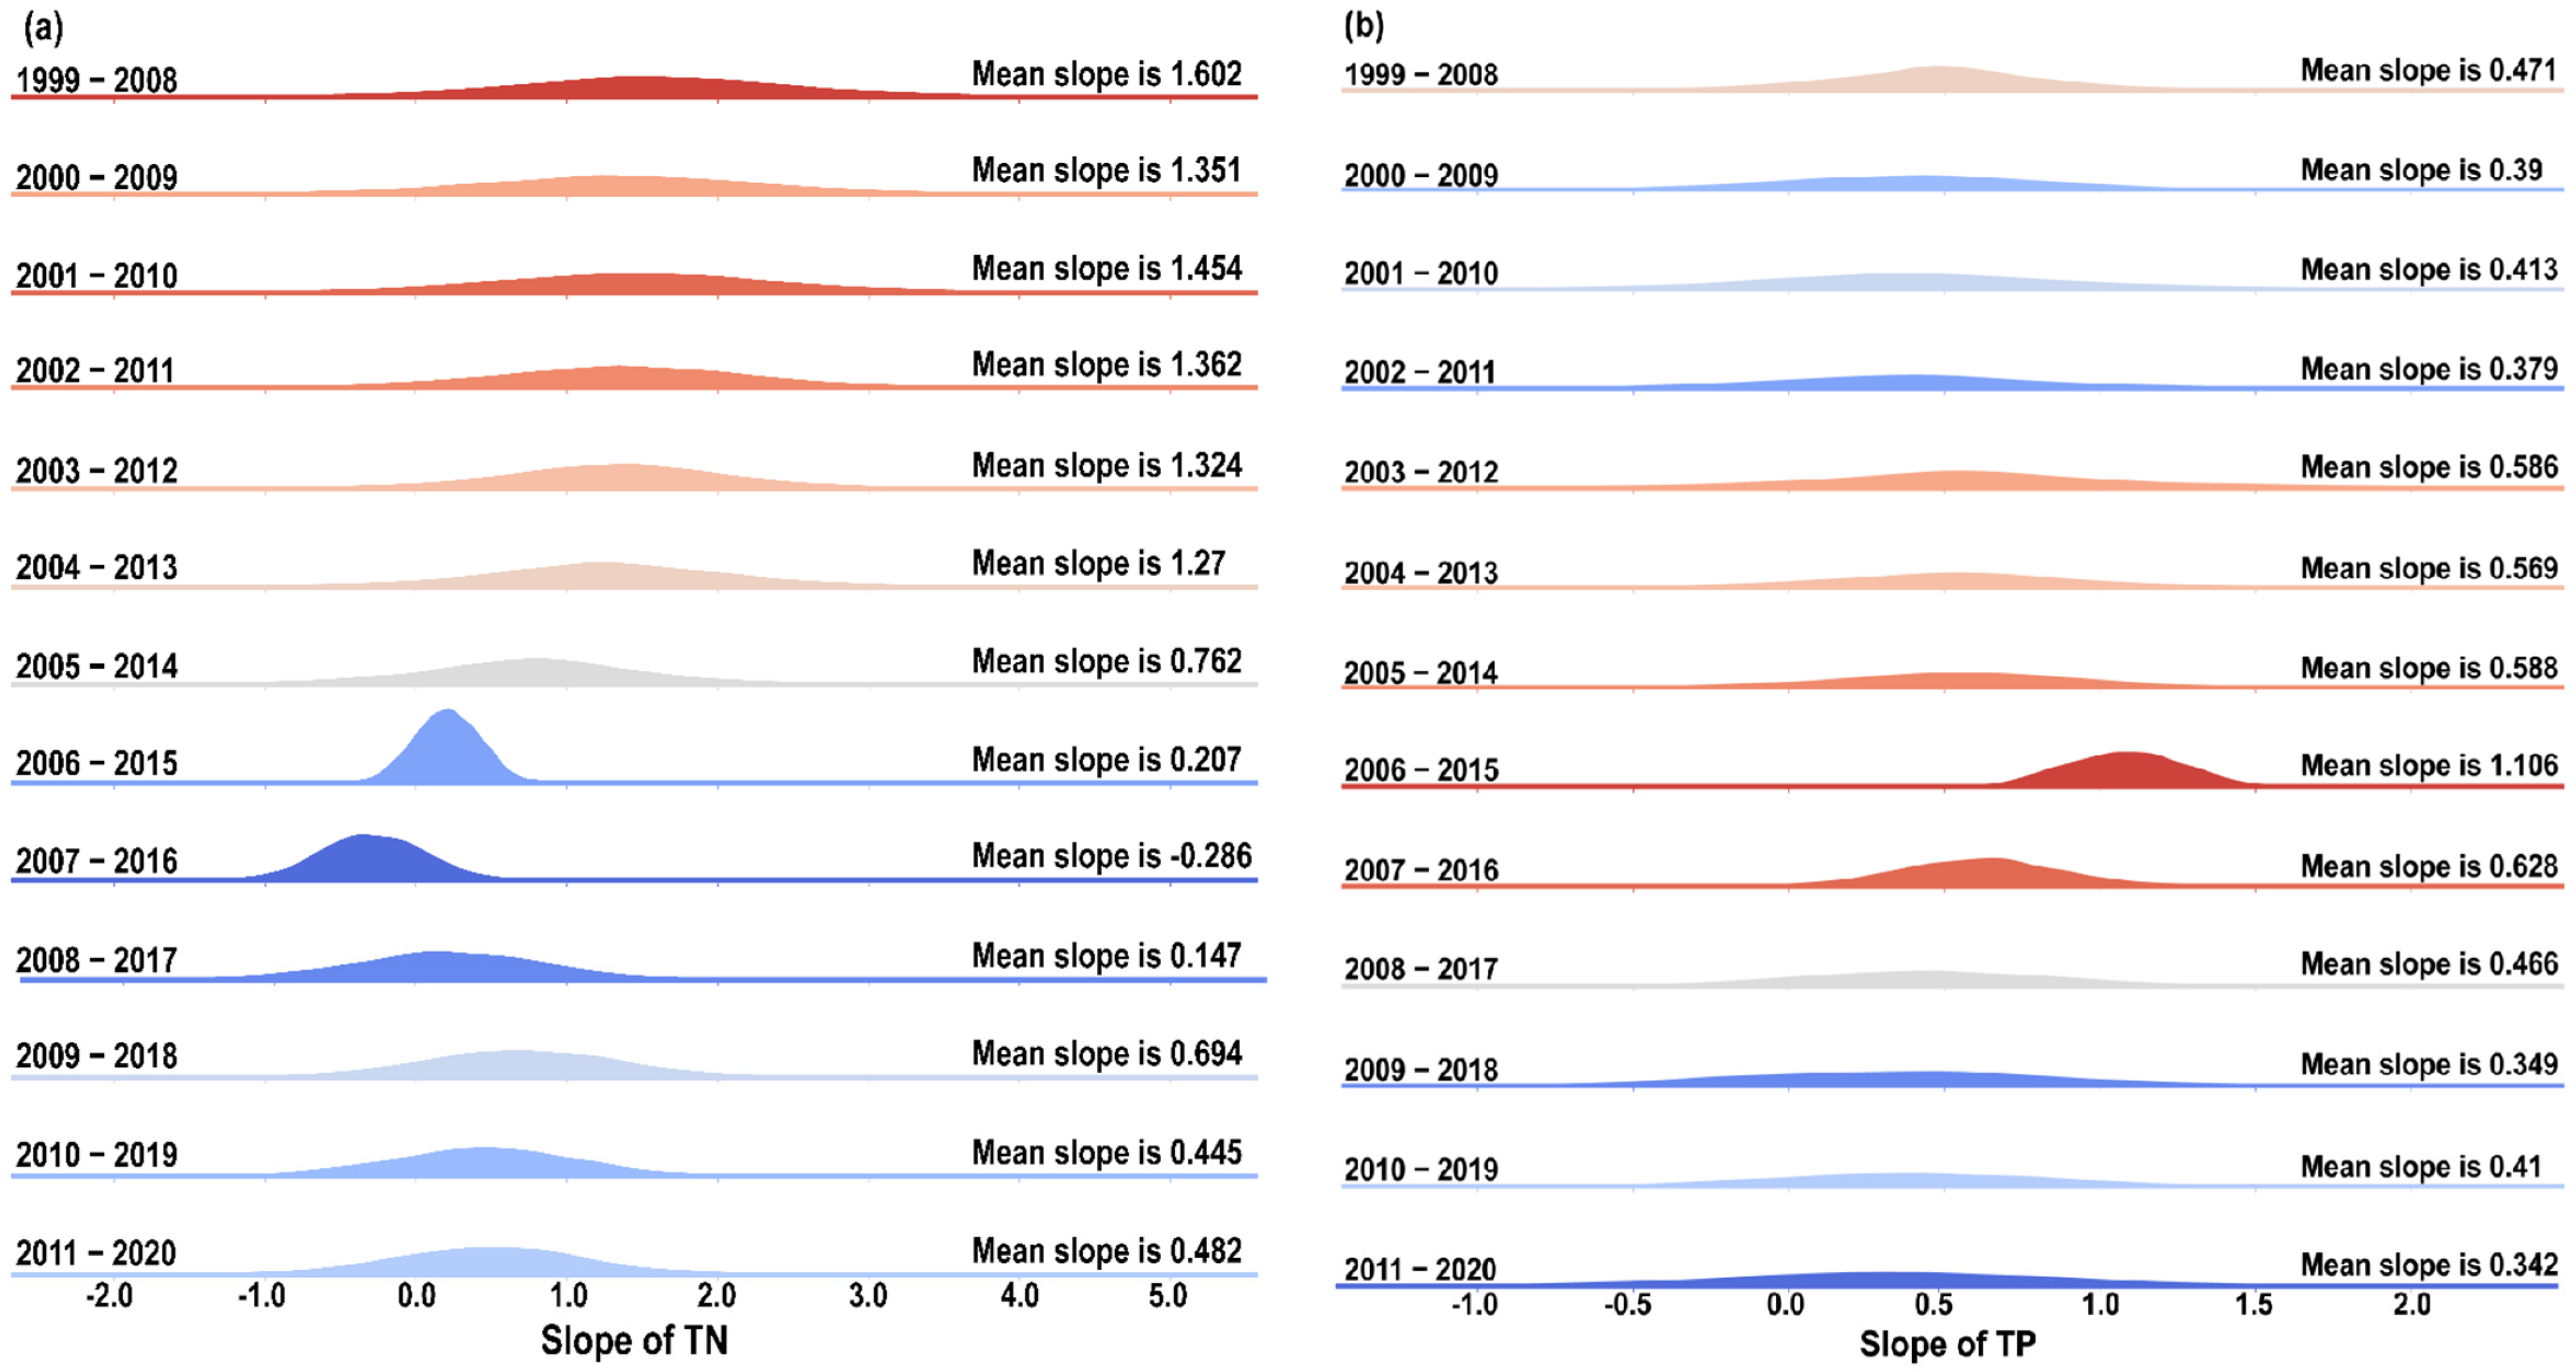
A 10-year moving window averaging approach (e.g., annual average slope trends for 1999–2008, 2000–2009, etc.) for the years 1999–2020 was selected for the analysis by means of HBGLMs, and the parameters obtained for each year in the HBGLMs are shown in Figure 4a,b. Sliding window averaging was performed, dividing 12 periods in year order, each corresponding to a 10-year rolling window (e.g., 1999–2008, 2000–2009, and so forth). The average slope values for each period are indicated on the right-hand side.
The distribution of the average TN slope of Lake Dianchi during different periods in summer is shown in Figure 4a. From 1999 to 2008 and all the way to 2011 and to 2020, the overall trend of TN changes over different periods was revealed as follows: (1) The average TN slope of Lake Dianchi in summer from 1999 to 2008 was the highest, reaching a maximum value of 1.602, indicating a significant increasing trend. From 2006 to 2015 to 2008 to 2017, the average TN slope in summer decreased, and the growth pole gradually changed to a low value distribution. (2) During the period from 2007 to 2016, the average TN slope in summer decreased to the minimum value and reached a negative value of −0.286, indicating a rapid decline. From 2006 to 2015 to 2008 to 2017, the average TN slope in summer decreased, and the growth rate slowed to a low value distribution. (3) During the three periods from 2009 to 2018 to 2011 to 2020, the average TN slope in summer recovered to some extent, but the overall growth rate was not as good as that during the previous periods. The average TN slopes in summer were relatively concentrated during the two periods of 2005–2014 and 2008–2017, and the variation amplitudes were relatively stable. (4) During the period from 2009 to 2020, the average TN slope in summer recovered to a slightly positive value but was much lower than the early peak value.
The fluctuating changes in the average slope of the TP in summer are shown in Figure 4b. The average TP slope in summer first tended to increase but then decreased. During the periods of 2006–2015 and 2007–2016, the average TP slope in summer significantly increased to the maximum value of 1.106 and then gradually decreased. The slopes during the periods of 2003–2012, 2005–2014 and 2007–2016 were also relatively high, and the growth trend of the average TP slope in summer was more obvious. During the periods of 2010–2019 and 2011–2020, the slope of the average TP in summer was relatively stable, with a slight rebound, but did not return to the early high level, indicating that the slope of the average TP in summer fluctuated gradually and tended to be stable. The average TP slope in summer peaked between 2006 and 2015, whereas the average slope decreased during recent periods (such as 2011–2020), indicating that the growth of the average TP slope tended to be stable.
In comparison, during the period from 1999 to 2006, the average slopes of TN and TP in Lake Dianchi in summer both showed a downward trend. However, the slopeN of Lake Dianchi was still much greater than the slopeP. At this time, the nutrient pattern of Lake Dianchi was N restricted. From 2006–2015 to 2008–2017, the average TN slope in summer was low, while the average TP slope in summer significantly increased to a maximum value of 1.106 during this period but then gradually decreased, much more than that in other periods, resulting in slopeP being greater than slopeN. At this time, the nutritional mode of Lake Dianchi changed from the original N-restricted nutritional mode to P-restricted, with the lake becoming a P-restricted lake. The average TN slope in summer during the three periods from 2009 to 2020 slightly increased but was much lower than that in the early stage. The average TP slope in summer tended to be flat during these three periods, and the nutrient pattern of Lake Dianchi transformed into one where both nitrogen and phosphorus were restricted [1,53]. During the nitrogen and phosphorus restriction periods (the three periods from 2009 to 2020), the increase in nitrogen accelerated the growth of phytoplankton and the absorption of phosphorus [1]. With the sinking and death of phytoplankton, phosphorus and organic matter are carried into lake sediments. This process reduces the phosphorus in the lake, resulting in a relatively insufficient demand for phosphorus in the lake. Therefore, the lake has reached the P limit. The analysis of the average slope change in summer shown in Figure 4 and the TN/TP trend shown in Figure 3 reveal that the future nutritional pattern of Lake Dianchi will gradually shift from being restricted by both nitrogen and phosphorus to being dominated by phosphorus, indicating that phosphorus is an important factor in managing large-scale eutrophication.

4. Discussion

4.1. Time-Varying Nutrient Limitation Revealed by 22-Year Evidence

Our 22-year HBGLM framework with 10-year moving windows shows that summertime slopes relating Chla to TN and TP evolved through three phases: early N-leaning limitation (1999–2006), a mid-period P-leaning phase (peaking in 2006–2015 windows), and recent colimitation with a gradual shift back towards P-sensitivity (2011–2020). During the P restriction period (in 2007, 2013, and 2017), the increase in P accelerated the growth of phytoplankton and the absorption of N. When phytoplankton sank and died, they carried N and organic matter into the lake sediments. This process reduced the nitrogen content in the lake, resulting in a relative nitrogen deficiency. In the coming years, the nutritional pattern of Dianchi Lake will gradually shift from being restricted by both nitrogen and phosphorus to being dominated by phosphorus restriction (Figure 4). This time-varying limitation aligns with multi-lake evidence that chlorophyll–nutrient relationships depend on the trophic state and evolve over multiyear windows: global and shallow-lake syntheses find robust long-term stoichiometric links, but with the TN vs. TP influence shifting across TN:TP windows and quantiles of Chla. Recent quantile regression analyses across lakes further indicate that TP is dominant at high Chla quantiles, particularly where phytoplankton biomass is elevated—which is consistent with our mid-to-late period P sensitivity [17,54]. In addition, environmental factors such as lake depth, Secchi, and hydrology significantly modulate how nutrients are translated into Chla. This explains why this shallow and regulated lake in Dianchi switched between N and P and other limitations over time [52].
Lake Dianchi is a typical semi-enclosed lake with a relatively deep average water depth (5.4 m), long retention time (3.5 years), and long eutrophication history and is conducive to weak nitrification–denitrification coupling and high net N accumulation. The experimentally measured Chla concentration in Lake Dianchi was much higher than that in Taihu Lake (annual mean value of 21.75 μg·L−1 from 2007 to 2017) [5,16,55]. The dynamic changes in the relative importance of N and P to the growth of algae in Lake Dianchi and the occurrence of continuous colimitation of N and P are consistent with the recent trend of nutrient limitation patterns in eutrophic lakes worldwide. According to previous reports, as knowledge on nutrient limitation in aquatic systems has increased, evidence of “parallel” N limitation (such as N and P limitation) or “sequential” nutrient limitation (two nutrients where one is limiting and the other is releasing) has increased in lakes and marine systems [10,21]. A long-term shift towards stronger P control occurs when external N declines faster than P or when internal P persists in eutrophic lakes, which is consistent with our late-window P-leaning response [45,52]. Eutrophic lakes generally have common limitations, and the TN:TP indicators conform to the long-term inference methodology for shallow lakes [17,46]. A long-term shift towards stronger P control occurs when external N declines faster than P or when internal P persists in eutrophic lakes, which is consistent with our late-window P-leaning response [5,52]. Eutrophic lakes generally have common limitations, and the TN:TP indicators conform to the long-term inference methodology for shallow lakes [17,27]. During early windows (1999–2006), our analysis suggested relatively stronger N leverage, whereas many global syntheses emphasize P control in oligotrophic and mesotrophic states and co-control in eutrophic states. We attribute this discrepancy to the Dianchi-specific context: fast N removal via denitrification vs. sediment P retention can cause transient N limitation, while TP remains buffered by internal stores [23,25]. Hydrodynamics and water diversion altered residence time and stratification patterns in Waihai, shifting how nutrient pools translated into Chla [56]. Warming-enhanced internal P release can amplify TP availability over time, altering the apparent balance of limitations [57,58].

4.2. Mechanistic Drivers: Hydrodynamics and Internal Loading Restructuring N-P-Chla Coupling

P is retained while N is preferentially removed by denitrification in shallow lakes, making P the more persistent driver after external-load reductions; this matches the observed shift towards P sensitivity in late windows [59,60]). Recent PCLake+ modelling for Lake Dianchi quantified critical TN:TP load thresholds for regime shifts and revealed that hydrological manipulation (water level/inflow) can increase restoration thresholds, facilitating transitions towards macrophyte-dominated clear states—mechanistically linking hydrodynamics with nutrient thresholds [61]. In Waihai, a coupled hydrodynamic–water quality model demonstrated that diversion timing, inlet, and outlet placement and increased diversion volume significantly improved water quality, providing evidence that flow reconfiguration can restructure nutrient–Chla coupling [56]. Concurrently, warming enhances internal P loading by extending stratification, deoxygenating bottom waters and accelerating mineralization, explaining why Dianchi remains P-responsive despite external controls [57]. Moreover, studies focusing on plateau lakes (including Dianchi Lake) have shown that endogenous P release is highly responsive to 50-year temperature variability, reinforcing the warming–internal-P pathway in high-elevation systems [58]. Complementarily, the antagonistic vs. synergistic interactions between warming and TN:TP vary across different nutrient input scenarios, showing antagonistic or synergistic effects, suggesting that in the context of warming, simultaneous control of nitrogen and phosphorus is necessary [62].

4.3. Management Implications and Limitations

N and P are important nutrients in lakes. Their excessive accumulation (exceeding the self-purification capacity of the lake) may lead to eutrophication, which in turn can cause problems such as algal blooms. These results underscore the integrated nature of nutrient flows among external inputs, internal cycling, and ecological responses in Lake Dianchi and highlight the need to implement integrated management at the watershed scale. External and internal loading indicate that the patterns for controlling lake eutrophication are closely related to basin inputs and lake responses. Therefore, a single management measure (such as reducing internal loading or limiting external loading) is ineffective [63,64]. This traceability suggests that we should embrace the ‘modes of thinking and doing’ of integrated management of ‘mountains, rivers, forests, farmlands, lakes and grasslands’ (mo shan zhi liu, mo shan zhi ye, mo mu zhi dou, mo hai zhi yu, mo tuan zhi tian, mo tuo zhi di), reducing internal loads inside lakes, controlling external allochthon inputs, and considering the interactions between terrestrial and aquatic ecosystems to maintain the health of watershed-lake ecosystems [65,66].
P remains the lever for long-term recovery, given (i) persistent internal P stores and (ii) warming-enhanced internal P release [24,60]. Hydrodynamic reconfiguration can increase water exchange, reduce residence time, and increase effective restoration thresholds alongside external loading cuts [67]. Because Chla–nutrient conversion varies with depth, clarity, and hydrology, dual-nutrient management remains prudent under warming [52]. To reasonably assess the nutrient limitation status of lakes, more empirical studies on algal physiology and community biogeochemical dynamics along an N–P ratio gradient are needed to provide the most fundamental data, if not a complete mechanistic understanding, of the role of nutrient limitation in the structuring and functioning of lakes. Numerical tools, such as lake ecosystem process models, are also needed to complement the empirical analysis and dynamically simulate the effects of N and P nutrient limitations on the structure and function of ecosystems [68,69].

5. Conclusions

The Chla and TP concentrations decreased by 49% and 78%, respectively. The TN:TP ratio (by mass) was used as an indicator of potential nutrient limitation in the lake. Internal nutrient cycling influences nutrient concentrations, which in turn affect phytoplankton and algal biomass, reflecting the nutrient relationships among N, P, and Chla. Nutrient limitation variability was observed as follows: between 1999 and 2020, Lake Dianchi evolved from N limitation to N and P colimitation, and in recent years, it has tended towards P sensitivity, which is consistent with the evolution of the relative importance of TN and TP to Chla during different periods, as obtained by the HBGLM. This finding is consistent with evidence from large-scale studies of the generalization of colimitation in eutrophic lakes and the dominance of TP at high Chla levels. In certain years (such as 2007, 2013, and 2017), the variations were in line with the long-term trends of TN:TP and the distributions of the average slopes of TN and TP across different periods. These years primarily exhibited patterns of colimitation by N and P or P limitation, indirectly confirming that Lake Dianchi will transition from N and P colimitation to being primarily limited by P.
Mechanistic restructuring by hydrodynamics and internal loading were observed as follows: persistent internal P and hydrodynamic modifications jointly modulate effective nutrient–Chla coupling and restoration thresholds. N is the primary limiting nutrient element in most cases, whereas P is the most significant nutrient element contributing to water eutrophication. Recovery is more likely when dual-nutrient (N + P) control is combined with internal P suppression (e.g., oxygenation, in situ P control/passivation) and operational hydrology to shorten the residence time and suppress the resuspension and hypoxia risks.
Long-term fractionated nutrient species (DIN, DON, SRP, DOP, and PP) are sparse; future work should integrate process experiments and causal-based models with monitoring to quantify thresholds and evaluate regime-shift risks under warming and variable inflows. Stage-dependent control and the need for dual-nutrient plus internal-load management are likely transferable to other shallow, regulated eutrophic lakes experiencing climatic and hydrological variability.

Author Contributions

Conceptualization, L.Z. and Y.H.; methodology, K.Z., B.D. and J.W.; Data curation, K.Z., B.D. and J.W.; writing—original draft, K.Z.; writing—review and editing, L.Z.; supervision, L.Z. and Y.H.; Other, T.L., Y.C., Q.P. and Q.Z. All authors have read and agreed to the published version of the manuscript.

Funding

This project was supported by the Young and Middle-Aged Academic and Technological Leaders of Yunnan (No. 202405AC350070).

Data Availability Statement

All data generated or analysed during this study are included in this article. The original data has been explained in the paper.

Acknowledgments

The authors are grateful to the Kunming Environmental Monitoring Center (KEMC) for providing the input data for this study.

Conflicts of Interest

The authors declare that they have no known competing financial interests or personal relationships that could have appeared to influence the work reported in this paper.

References

  1. Wu, Z.; Liu, Y.; Liang, Z.; Wu, S.; Guo, H. Internal cycling, not external loading, decides the nutrient limitation in eutrophic lake: A dynamic model with temporal Bayesian hierarchical inference. Water Res. 2017, 116, 231–240. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  2. Xu, H.; Paerl, H.W.; Qin, B.Q.; Zhu, G.W.; Gaoa, G. Nitrogen and phosphorus inputs control phytoplankton growth in eutrophic Lake Taihu, China. Limnol. Oceanogr. 2010, 55, 420–432. [Google Scholar] [CrossRef] [Scilit]
  3. Conley, D.J.; Paerl, H.W.; Howarth, R.W.; Boesch, D.F.; Seitzinger, S.P.; Havens, K.E.; Lancelot, C.; Likens, G.E. Controlling Eutrophication: Nitrogen and Phosphorus. Science 2009, 323, 1014–1015. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  4. Qian, R.; Wang, X.; Gao, J.; Yang, H.; Han, J.; Zhang, Q.; Yan, R.; Liao, K.; Huang, J. A modelling framework to track phosphorus sources of the drinking water intakes in a large eutrophic lake. J. Hydrol. 2022, 607, 127564. [Google Scholar] [CrossRef] [Scilit]
  5. Qin, B.Q.; Paerl, H.W.; Brookes, J.D.; Liu, J.G.; Jeppesen, E.; Zhu, G.W.; Zhang, Y.L.; Xu, H.; Shi, K.; Deng, J.M. Why Lake Taihu continues to be plagued with cyanobacterial blooms through 10 years (2007–2017) efforts. Sci. Bull. 2019, 64, 354–356. [Google Scholar] [CrossRef] [Scilit]
  6. Paerl, H.W.; Havens, K.E.; Xu, H.; Zhu, G.; McCarthy, M.J.; Newell, S.E.; Scott, J.T.; Hall, N.S.; Otten, T.G.; Qin, B. Mitigating eutrophication and toxic cyanobacterial blooms in large lakes: The evolution of a dual nutrient (N and P) reduction paradigm. Hydrobiologia 2020, 847, 4359–4375. [Google Scholar] [CrossRef] [Scilit]
  7. Schindler, D.W. The dilemma of controlling cultural eutrophication of lakes. Proc. Biol. Sci. 2012, 279, 4322–4333. [Google Scholar] [CrossRef] [Scilit]
  8. Carpenter, S.R. Phosphorus control is critical to mitigating eutrophication. Proc. Natl. Acad. Sci. USA 2008, 105, 11039–11040. [Google Scholar] [CrossRef] [Scilit]
  9. Schindler, D.W.; Hecky, R.E.; Findlay, D.L.; Stainton, M.P.; Parker, B.R.; Paterson, M.J.; Beaty, K.G.; Lyng, M.; Kasian, S.E.M. Eutrophication of lakes cannot be controlled by reducing nitrogen input: Results of a 37-year whole-ecosystem experiment. Proc. Natl. Acad. Sci. USA 2008, 105, 11254–11258. [Google Scholar] [CrossRef] [Scilit]
  10. Paerl, H.W.; Gardner, W.S.; Havens, K.E.; Joyner, A.R.; McCarthy, M.J.; Newell, S.E.; Qin, B.; Scott, J.T. Mitigating cyanobacterial harmful algal blooms in aquatic ecosystems impacted by climate change and anthropogenic nutrients. Harmful Algae 2016, 54, 213–222. [Google Scholar] [CrossRef] [Scilit]
  11. Scott, J.T.; McCarthy, M.J. Nitrogen fixation may not balance the nitrogen pool in lakes over timescales relevant to eutrophication management. Limnol. Oceanogr. 2010, 55, 1265–1270. [Google Scholar] [CrossRef] [Scilit]
  12. Wang, H.J.; Wang, H.Z. Mitigation of lake eutrophication: Loosen nitrogen control and focus on phosphorus abatement. Prog. Nat. Sci. 2009, 19, 1445–1451. [Google Scholar] [CrossRef] [Scilit]
  13. Elser, J.J.; Andersen, T.; Baron, J.S.; Bergström, A.K.; Jansson, M.; Kyle, M.; Nydick, K.R.; Steger, L.; Hessen, D.O. Shifts in Lake N:P Stoichiometry and Nutrient Limitation Driven by Atmospheric Nitrogen Deposition. Science 2009, 326, 835–837. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  14. Liang, Z.; Soranno, P.A.; Wagner, T. The role of phosphorus and nitrogen on chlorophyll a: Evidence from hundreds of lakes. Water Res. 2020, 185, 116236. [Google Scholar] [CrossRef] [Scilit]
  15. Zhao, L.; Zhu, R.; Zhou, Q.; Jeppesen, E.; Yang, K. Trophic status and lake depth play important roles in determining the nutrient-chlorophyll a relationship: Evidence from thousands of lakes globally. Water Res. 2023, 242, 120182. [Google Scholar] [CrossRef] [Scilit]
  16. Qin, B.; Zhou, J.; Elser, J.J.; Gardner, W.S.; Deng, J.; Brookes, J.D. Water Depth Underpins the Relative Roles and Fates of Nitrogen and Phosphorus in Lakes. Environ. Sci. Technol. 2020, 54, 3191–3198. [Google Scholar] [CrossRef] [Scilit]
  17. Graeber, D.; McCarthy, M.J.; Shatwell, T.; Borchardt, D.; Jeppesen, E.; Søndergaard, M.; Lauridsen, T.L.; Davidson, T.A. Consistent stoichiometric long-term relationships between nutrients and chlorophyll-a across shallow lakes. Nat. Commun. 2024, 15, 809. [Google Scholar] [CrossRef] [Scilit]
  18. Nowlin, W.H.; Evarts, J.L.; Vanni, M.J. Release rates and potential fates of nitrogen and phosphorus from sediments in a eutrophic reservoir. Freshw. Biol. 2005, 50, 301–322. [Google Scholar] [CrossRef] [Scilit]
  19. McLauchlan, K.K.; Williams, J.J.; Craine, J.M.; Jeffers, E.S. Changes in global nitrogen cycling during the Holocene epoch. Nature 2013, 495, 352–355. [Google Scholar] [CrossRef] [Scilit]
  20. Ding, Y.; Xu, H.; Deng, J.; Qin, B.; He, Y. Impact of nutrient loading on phytoplankton: A mesocosm experiment in the eutrophic Lake Taihu, China. Hydrobiologia 2019, 829, 167–187. [Google Scholar] [CrossRef] [Scilit]
  21. Xu, T.; Yang, T.; Xiong, M. Time scales of external loading and spatial heterogeneity in nutrients-chlorophyll a response: Implication on eutrophication control in a large shallow lake. Ecol. Eng. 2020, 142, 105636. [Google Scholar] [CrossRef] [Scilit]
  22. Lawson, G.M.; Young, J.L.; Aanderud, Z.T.; Jones, E.F.; Bratsman, S.; Daniels, J.; Malmfeldt, M.P.; Baker, M.A.; Abbott, B.W.; Daly, S.; et al. Nutrient limitation and seasonality associated with phytoplankton communities and cyanotoxin production in a large, hypereutrophic lake. Harmful Algae 2025, 143, 102809. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  23. Schindler, D.W.; Hecky, R.E.; McCullough, G.K. The rapid eutrophication of Lake Winnipeg: Greening under global change. J. Great Lakes Res. 2012, 38, 6–13. [Google Scholar] [CrossRef] [Scilit]
  24. Jeppesen, E.; Sorensen, P.B.; Johansson, L.S.; Sondergaard, M.; Lauridsen, T.L.; Nielsen, A.; Mejlhede, P. Recovery of lakes from eutrophication: Changes in nitrogen retention capacity and the role of nitrogen legacy in 10 Danish lakes studied over 30 years. Hydrobiologia 2025, 852, 377–387. [Google Scholar] [CrossRef] [Scilit]
  25. Bruesewitz, D.A.; Tank, J.L.; Hamilton, S.K. Incorporating spatial variation of nitrification and denitrification rates into whole-lake nitrogen dynamics. J. Geophys. Res. Biogeosci. 2012, 117, G00N07. [Google Scholar] [CrossRef] [Scilit]
  26. Li, Y.; Jin, H.; Chen, J.; Wang, D.; Yang, Z.; Wang, B.; Zhuang, Y.; Wang, R. Nitrogen removal through sediment denitrification in the Yangtze Estuary and its adjacent East China Sea: A nitrate limited process during summertime. Sci. Total Environ. 2021, 795, 148616. [Google Scholar] [CrossRef] [Scilit]
  27. Qin, B.; Zhang, Y.; Zhu, G.; Gao, G. Eutrophication control of large shallow lakes in China. Sci. Total Environ. 2023, 881, 163494. [Google Scholar] [CrossRef] [Scilit]
  28. Peng, X.; Zhang, L.; Li, Y.; Lin, Q.; He, C.; Huang, S.; Li, H.; Zhang, X.; Liu, B.; Ge, F.; et al. The changing characteristics of phytoplankton community and biomass in subtropical shallow lakes: Coupling effects of land use patterns and lake morphology. Water Res. 2021, 200, 117235. [Google Scholar] [CrossRef] [Scilit]
  29. Liu, X.; Wang, H. Dianchi Lake, China: Geological formation, causes of eutrophication and recent restoration efforts. Aquat. Ecosyst. Health Manag. 2016, 19, 40–48. [Google Scholar] [CrossRef] [Scilit]
  30. Rankenhohn, F.; Strauß, T.; Wermter, P. Dianchi Shallow Lake Management. In Chinese Water Systems: Volume 4: Applied Water Management in China; Dohmann, M., Grambow, M., Song, Y., Wermter, P., Eds.; Springer International Publishing: Cham, Switzerland, 2022; pp. 69–102. [Google Scholar]
  31. Wang, Q.; Xiao, X.; Yao, A.; Hillman, A.L.; Jiang, Z.; Wang, R.; Yang, X. Unraveling the early human impacts on the ecosystem of Dianchi Lake: A 20,000-year diatom record from the southeastern Tibetan Plateau. Quat. Sci. Rev. 2024, 337, 108813. [Google Scholar] [CrossRef] [Scilit]
  32. Li, X.; Janssen, A.B.G.; de Klein, J.J.M.; Kroeze, C.; Strokal, M.; Ma, L.; Zheng, Y. Modeling nutrients in Lake Dianchi (China) and its watershed. Agric. Water Manag. 2019, 212, 48–59. [Google Scholar] [CrossRef] [Scilit]
  33. Beck, M.W.; de Valpine, P.; Murphy, R.; Wren, I.; Chelsky, A.; Foley, M.; Senn, D.B. Multi-scale trend analysis of water quality using error propagation of generalized additive models. Sci. Total Environ. 2022, 802, 149927. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  34. Geng, Y.; Cao, Z.; Yu, R.; Li, X.; Sun, H.; Wang, X. Delving into nitrogen and phosphorus dynamics in shallow eutrophic lakes: Multi-interface response to freeze-thaw cycles. Sci. Total Environ. 2024, 955, 177052. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  35. Liu, Y.; Jiang, Q.; Sun, Y.; Jian, Y.; Zhou, F. Decline in nitrogen concentrations of eutrophic Lake Dianchi associated with policy interventions during 2002–2018. Environ. Pollut. 2021, 288, 117826. [Google Scholar] [CrossRef] [Scilit]
  36. Duan, Z.; Gao, W.; Cheng, G.; Zhang, Y.; Chang, X. Warming surface and Lake heatwaves as key drivers to harmful algal Blooms: A case study of Lake Dianchi, China. J. Hydrol. 2024, 632, 130971. [Google Scholar] [CrossRef] [Scilit]
  37. Deng, J.; Shan, K.; Shi, K.; Qian, S.S.; Zhang, Y.; Qin, B.; Zhu, G. Nutrient reduction mitigated the expansion of cyanobacterial blooms caused by climate change in Lake Taihu according to Bayesian network models. Water Res. 2023, 236, 119946. [Google Scholar] [CrossRef] [Scilit]
  38. Li, H.; Zhang, H.; Duan, L.; Liu, Q.; Li, D.; Huang, J.; Fu, J.; Zi, L.; Xu, T. Spatiotemporal variations in water quality parameters and assessment of the current status and challenges of eutrophication in Lake Dian. Ecol. Indic. 2025, 177, 113821. [Google Scholar] [CrossRef] [Scilit]
  39. Kovalenko, K.E.; Reavie, E.D.; Barbiero, R.P.; Burlakova, L.E.; Karatayev, A.Y.; Rudstam, L.G.; Watkins, J.M. Patterns of long-term dynamics of aquatic communities and water quality parameters in the Great Lakes: Are they synchronized? J. Great Lakes Res. 2018, 44, 660–669. [Google Scholar] [CrossRef] [Scilit]
  40. Zhao, K.; Wulder, M.A.; Hu, T.; Bright, R.; Wu, Q.; Qin, H.; Li, Y.; Toman, E.; Mallick, B.; Zhang, X.; et al. Detecting change-point, trend, and seasonality in satellite time series data to track abrupt changes and nonlinear dynamics: A Bayesian ensemble algorithm. Remote Sens. Environ. 2019, 232, 111181. [Google Scholar] [CrossRef] [Scilit]
  41. Yang, R.; Wu, J.; Zhao, J.; Guan, Q.; Fan, X.; Zhao, L. Marked interannual variability in the relative dominance of phytoplankton over submerged macrophytes rather than regime shifts in a shallow eutrophic lake: Evidence from long-term observations. Ecol. Indic. 2024, 166, 112301. [Google Scholar] [CrossRef] [Scilit]
  42. Mulverhill, C.; Coops, N.C.; Achim, A. Continuous monitoring and sub-annual change detection in high-latitude forests using Harmonized Landsat Sentinel-2 data. ISPRS J. Photogramm. Remote Sens. 2023, 197, 309–319. [Google Scholar] [CrossRef] [Scilit]
  43. Lyu, R.; Zhao, W.; Pang, J.; Tian, X.; Zhang, J.; Wang, N. Towards a sustainable nature reserve management: Using Bayesian network to quantify the threat of disturbance to ecosystem services. Ecosyst. Serv. 2022, 58, 101483. [Google Scholar] [CrossRef] [Scilit]
  44. Li, J.; Li, Z.-L.; Wu, H.; You, N. Trend, seasonality, and abrupt change detection method for land surface temperature time-series analysis: Evaluation and improvement. Remote Sens. Environ. 2022, 280, 113222. [Google Scholar] [CrossRef] [Scilit]
  45. Zhao, L.; Su, Y.; Gao, W.; Zhang, K.; Wu, J. Delayed water quality response to external nutrient loading reduction: The role of internal nutrient loading in a shallow eutrophic lake over 20 years. Ecol. Indic. 2025, 177, 113731. [Google Scholar] [CrossRef] [Scilit]
  46. Paerl, H.W.; Scott, J.T.; McCarthy, M.J.; Newell, S.E.; Gardner, W.S.; Havens, K.E.; Hoffman, D.K.; Wilhelm, S.W.; Wurtsbaugh, W.A. It Takes Two to Tango: When and Where Dual Nutrient (N & P) Reductions Are Needed to Protect Lakes and Downstream Ecosystems. Environ. Sci. Technol. 2016, 50, 10805–10813. [Google Scholar] [CrossRef] [Scilit]
  47. Wang, C.; Liu, J.; Qiu, C.; Su, X.; Ma, N.; Li, J.; Wang, S.; Qu, S. Identifying the drivers of chlorophyll-a dynamics in a landscape lake recharged by reclaimed water using interpretable machine learning. Sci. Total Environ. 2024, 906, 167483. [Google Scholar] [CrossRef] [Scilit]
  48. García–Nieto, P.J.; García–Gonzalo, E.; Fernández, J.R.A.; Muñiz, C.D. Forecast of chlorophyll-a concentration as an indicator of phytoplankton biomass in El Val reservoir by utilizing various machine learning techniques: A case study in Ebro river basin, Spain. J. Hydrol. 2024, 639, 131639. [Google Scholar] [CrossRef] [Scilit]
  49. Karpowicz, M.; Kuczyńska-Kippen, N.; Sługocki, Ł.; Czerniawski, R.; Bogacka-Kapusta, E.; Ejsmont-Karabin, J. Trophic status index discrepancies as a tool for improving lake management: Insights from 160 Polish lakes. Sci. Total Environ. 2025, 981, 179581. [Google Scholar] [CrossRef] [Scilit]
  50. Spaulding, S.A.; Platt, L.R.C.; Murphy, J.C.; Covert, A.; Harvey, J.W. Chlorophyll a in lakes and streams of the United States (2005–2022). Sci. Data 2024, 11, 611. [Google Scholar] [CrossRef] [Scilit]
  51. Guildford, S.J.; Hecky, R.E. Total nitrogen, total phosphorus, and nutrient limitation in lakes and oceans: Is there a common relationship? Limnol. Oceanogr. 2000, 45, 1213–1223. [Google Scholar] [CrossRef] [Scilit]
  52. Naderian, D.; Noori, R.; Kim, D.; Jun, C.; Bateni, S.M.; Woolway, R.I.; Sharma, S.; Shi, K.; Qin, B.; Zhang, Y.; et al. Environmental controls on the conversion of nutrients to chlorophyll in lakes. Water Res. 2025, 274, 123094. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  53. Crowley, K.F.; McNeil, B.E.; Lovett, G.M.; Canham, C.D.; Driscoll, C.T.; Rustad, L.E.; Denny, E.; Hallett, R.A.; Arthur, M.A.; Boggs, J.L.; et al. Do Nutrient Limitation Patterns Shift from Nitrogen Toward Phosphorus with Increasing Nitrogen Deposition Across the Northeastern United States? Ecosystems 2012, 15, 940–957. [Google Scholar] [CrossRef] [Scilit]
  54. Han, H.; Yan, X.; Li, X.; Zhao, X.; Qiu, J.; Huang, Z.; Yan, X.; Xia, Y. Quantile regression reveals phosphorous overwhelms nitrogen in controlling high chlorophyll-a concentration in freshwater lakes. J. Hydrol. 2025, 654, 132845. [Google Scholar] [CrossRef] [Scilit]
  55. Qin, B.; Deng, J.; Shi, K.; Wang, J.; Brookes, J.; Zhou, J.; Zhang, Y.; Zhu, G.; Paerl, H.W.; Wu, L. Extreme climate anomalies enhancing Cyanobacterial Blooms in eutrophic Lake Taihu, China. Water Resour. Res. 2021, 57, e2020WR029371. [Google Scholar] [CrossRef] [Scilit]
  56. Zhou, X.-Q.; Shen, Y.-M.; Tang, J. Numerical modeling of water diversion impacts on water quality improvement in Lake Dianchi. Environ. Model. Softw. 2025, 187, 106375. [Google Scholar] [CrossRef] [Scilit]
  57. Kong, X.; Determann, M.; Andersen, T.K.; Barbosa, C.C.; Dadi, T.; Janssen, A.B.G.; Paule-Mercado, M.C.; Pujoni, D.G.F.; Schultze, M.; Rinke, K. Synergistic Effects of Warming and Internal Nutrient Loading Interfere with the Long-Term Stability of Lake Restoration and Induce Sudden Re-eutrophication. Environ. Sci. Technol. 2023, 57, 4003–4013. [Google Scholar] [CrossRef] [Scilit]
  58. Yan, C.; Xia, R.; Chen, Y.; Jiao, L.; Liu, X.; Yin, Y.; Hu, Q.; Zhang, K.; Li, L.; Liu, H. Endogenous phosphorus release from plateau lakes responds significantly to temperature variability over the last 50 years. J. Environ. Manag. 2024, 371, 123259. [Google Scholar] [CrossRef] [Scilit]
  59. Burson, A.; Stomp, M.; Greenwell, E.; Grosse, J.; Huisman, J. Competition for nutrients and light: Testing advances in resource competition with a natural phytoplankton community. Ecology 2018, 99, 1108–1118. [Google Scholar] [CrossRef] [Scilit]
  60. Schindler, D.W.; Carpenter, S.R.; Chapra, S.C.; Hecky, R.E.; Orihel, D.M. Reducing Phosphorus to Curb Lake Eutrophication is a Success. Environ. Sci. Technol. 2016, 50, 8923–8929. [Google Scholar] [CrossRef] [Scilit]
  61. Wu, D.; Cao, M.; Gao, W.; Duan, Z.; Zhang, Y. Simulating critical nutrient loadings of regime shift in the shallow plateau Lake Dianchi. Ecol. Model. 2024, 491, 110689. [Google Scholar] [CrossRef] [Scilit]
  62. Wu, D.; Cao, M.; Gao, W.; Duan, Z.; Hou, X.; Zhang, Y. Combined effects of nutrient loadings and warming on algal blooms in a plateau lake: Dianchi, China. Hydrobiologia 2025. [Google Scholar] [CrossRef] [Scilit]
  63. Ma, X.; Jiao, X.; Sha, Z.; Ding, F.; Li, Y.; Xu, W.; Tang, A.; Xia, X.; Fangmeier, A.; Liu, X. Characterization of atmospheric bulk phosphorus deposition in China. Atmos. Environ. 2022, 279, 119127. [Google Scholar] [CrossRef] [Scilit]
  64. Beusen, A.H.W.; Bouwman, A.F.; Van Beek, L.P.H.; Mogollon, J.M.; Middelburg, J.J. Global riverine N and P transport to ocean increased during the 20th century despite increased retention along the aquatic continuum. Biogeosciences 2016, 13, 2441–2451. [Google Scholar] [CrossRef] [Scilit]
  65. Paerl, H.W.; Xu, H.; Hall, N.S.; Zhu, G.W.; Qin, B.Q.; Wu, Y.L.; Rossignol, K.L.; Dong, L.H.; McCarthy, M.J.; Joyner, A.R. Controlling Cyanobacterial Blooms in Hypertrophic Lake Taihu, China: Will Nitrogen Reductions Cause Replacement of Non-N2 Fixing by N2 Fixing Taxa? PLoS ONE 2014, 9, e113123. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  66. Zhou, J.; Han, X.; Brookes, J.D.; Qin, B. High probability of nitrogen and phosphorus co-limitation occurring in eutrophic lakes. Environ. Pollut. 2022, 292, 118276. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  67. Wu, X.; Wang, Y.; Chang, Y.; Hao, Z.; Jiao, L.; Zhang, R. Research Progress on the Occurrence, Adsorption, and Release of Phosphorus in the Sediments of Dianchi Lake and Prospects for Its Control. Water 2025, 17, 1652. [Google Scholar] [CrossRef] [Scilit]
  68. Jeppesen, E.; Sondergaard, M.; Liu, Z.W. Lake Restoration and Management in a Climate Change Perspective: An Introduction. Water 2017, 9, 122. [Google Scholar] [CrossRef] [Scilit]
  69. Janssen, A.B.G.; van Wijk, D.; van Gerven, L.P.A.; Bakker, E.S.; Brederveld, R.J.; DeAngelis, D.L.; Janse, J.H.; Mooij, W.M. Success of lake restoration depends on spatial aspects of nutrient loading and hydrology. Sci. Total Environ. 2019, 679, 248–259. [Google Scholar] [CrossRef] [Scilit]
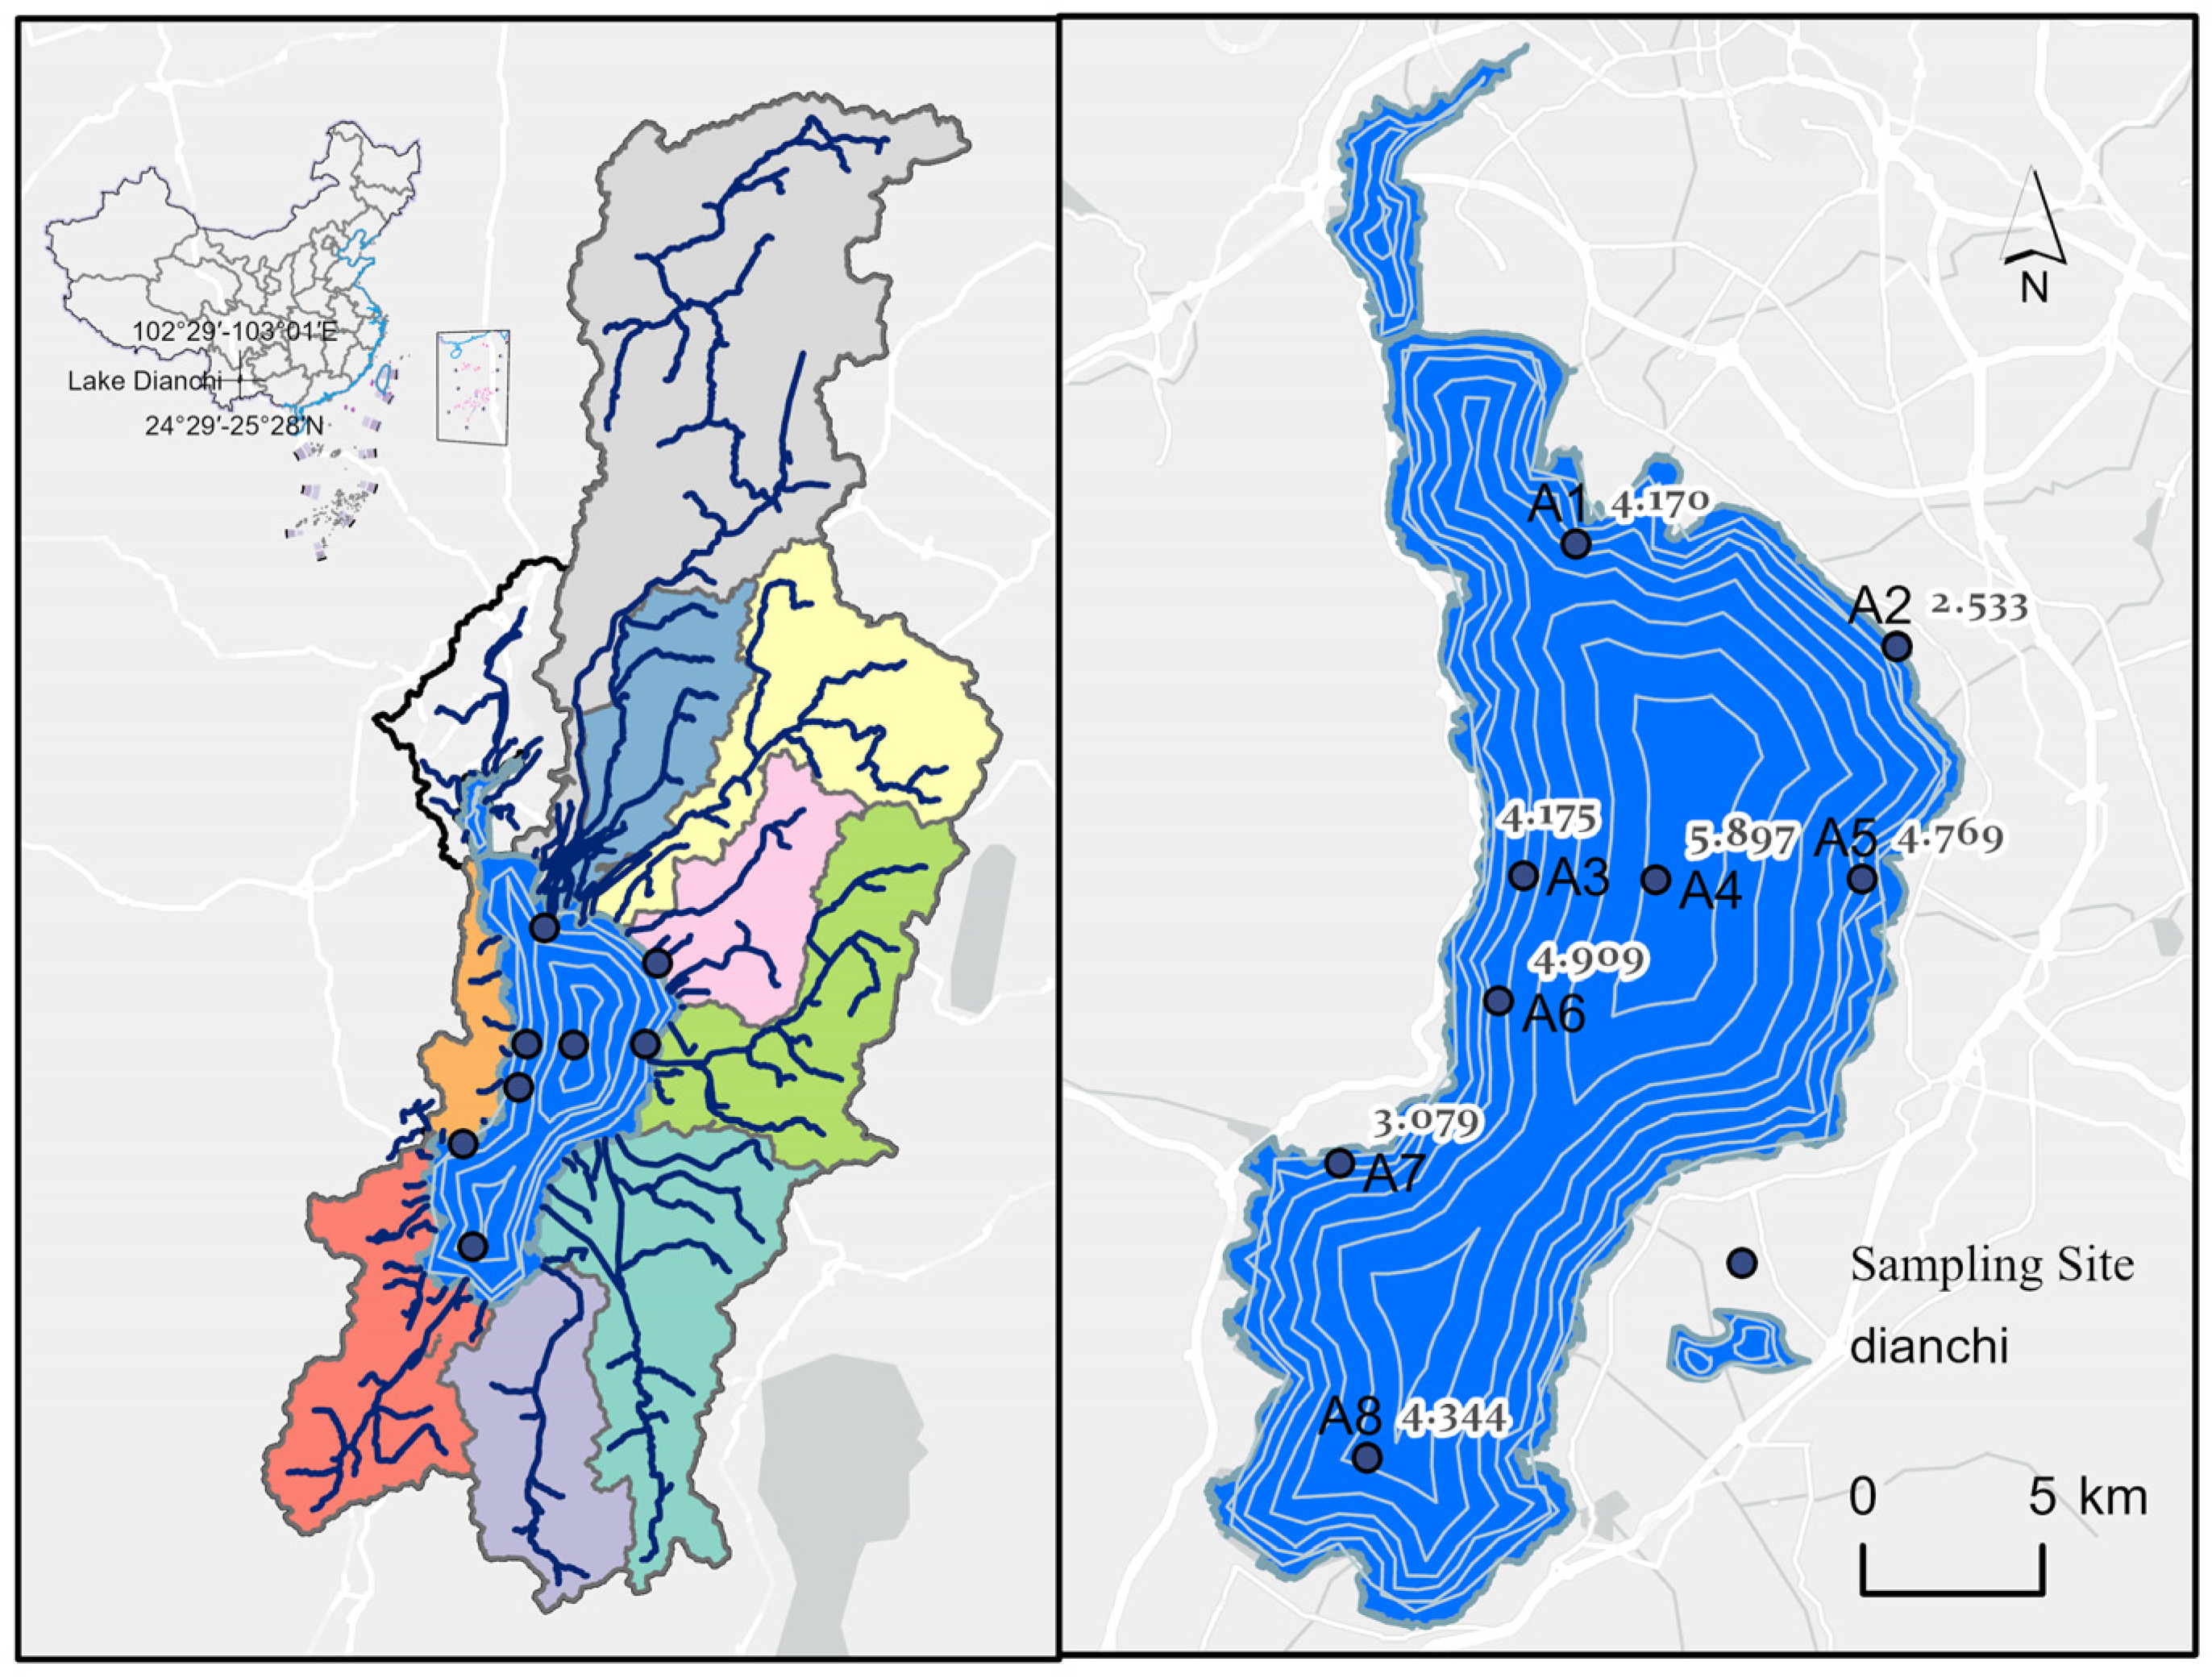
Figure 1. Location of Lake Dianchi in Southwest China and the distribution of the 8 sampling sites.
Water 17 02604 g001
Figure 2. Temporal variations in monthly average concentrations of TN (a), TP (b), and Chla (c) in Lake Dianchi from 1999 to 2020. Black dots represent means from eight monitoring stations, lines indicate temporal trends, and error bars show standard deviations across stations.
Water 17 02604 g002
Figure 3. Long-term Trends in Summer Nutrient Concentrations and TN:TP Ratios in Lake Dianchi from 1999 to 2020. (a) Summer total nitrogen (TN), (b) summer total phosphorus (TP), (c) summer chlorophyll-a (Chla) concentration, and (d) TN:TP mass ratios. Light purple transparent circles: Represent the monthly average values during the summer months (June, July, and August) for each year. Gray shaded areas indicate the distribution of bootstrap-sampled trends, with darker shades reflecting higher trend density and greater stability in those regions. Purple line denotes the median (50th percentile) of the bootstrap distribution, indicating the most probable trend trajectory. The overall extent of the gray shading represents the 95% confidence interval (from the 2.5th to the 97.5th percentiles), highlighting the statistical reliability of the trend estimates.
Water 17 02604 g003
Figure 4. (a) Distribution of the average slope of TN over different periods. There are 12 periods in annual order, each corresponding to a 10-year rolling window (e.g., 1999–2008, 2000–2009, and so on). The average slope value for each period is indicated on the right-hand side. (b) Distribution of the average slope of the TP over different periods. There are 12 periods in annual order, each corresponding to a 10-year rolling window (e.g., 1999–2008, 2000–2009, and so on). The average slope values for each period are indicated on the right-hand side.
Water 17 02604 g004
Table 1. Codes and coordinates of examined water-quality monitoring stations.
CodeSampling Point NameBasinDepth (m)LongitudeLatitude
A1Huiwanzhongnorthwest of Waihai4.17102.69024.914
A2Luojiayingnorthwest of Waihai2.533102.770102.770
A3Guanyinshanxinorthwest of Waihai4.175102.67624.838
A4Guanyinshanzhongnorthwest of Waihai5.897102.70924.837
A5Guanyinshandongeast of Waihai4.769102.76124.837
A6Baiyukounorthwest of Waihai4.909102.67024.810
A7Haikouxinorthwest of Waihai3.079102.63024.773
A8Dianchinansouth of Waihai4.344102.63624.706
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.