Article

Biocultural Productive Landscapes in the Andean–Amazon: Carbon, Biodiversity, and Livelihoods in Market-Linked Traditional Systems


by
Bolier Torres
1,2,*,
Cristhian Tipán-Torres
2,3,
Héctor Reyes
4,
Aracely Tapia
5,
Julio Muñoz-Rengifo
1,
Robinson Herrera-Feijoo
6 and
Antón García
7,*
1
Departamento de Silvicultura y Producción Agrícola, Universidad Estatal Amazónica (UEA), Pastaza 160101, Ecuador
2
Ochroma Consulting & Services, Tena 150150, Ecuador
3
Instituto Superior Tecnológico Ciudad de Valencia, Puebloviejo 120201, Ecuador
4
Dirección de Investigación, Posgrado, Vinculación y Transferencia de Tecnología, Universidad Estatal Amazónica (UEA), Pastaza 160101, Ecuador
5
Gobierno Provincial de Napo, Tena 150150, Ecuador
6
Facultad de Ciencias Agrarias y Forestales, Universidad Técnica Estatal de Quevedo (UTEQ), Quevedo Av. Quito Km, 1 1/2 Vía a Santo Domingo de los Tsáchilas, Quevedo 120550, Ecuador
7
Department of Animal Production, Faculty of Veterinary Sciences, University of Cordoba, 14071 Cordoba, Spain
*
Authors to whom correspondence should be addressed.
Sustainability 2026, 18(5), 2451; https://doi.org/10.3390/su18052451
Submission received: 12 January 2026 / Revised: 25 February 2026 / Accepted: 28 February 2026 / Published: 3 March 2026

Abstract

Tree-based production systems embedded within Amazonian biocultural landscapes remain systematically undervalued in global climate, biodiversity, and development policy frameworks. This study assessed tree diversity, structural attributes, and carbon stocks across traditional cacao-based Amazonian agroforestry systems (Chakra), tree-rich silvopastoral systems, and old-growth forests in the Andean–Amazon transition zone of Ecuador. Based on 28 sampling plots (DBH ≥ 10 cm), old-growth forests stored the highest aboveground carbon stocks, while agroforestry and silvopastoral systems retained approximately 20–30% of forest carbon, equivalent to ~100–180 Mg CO2-equivalent ha−1—far exceeding values reported for monocultures or treeless pastures. A total of 151 tree species were recorded across all land-use systems, with forests harboring the highest richness (122 species), followed by agroforestry (35 species) and silvopastoral systems (28 species). Carbon storage was highly concentrated in a limited subset of multifunctional species: in agroforestry systems, eight species accounted for ~80% of total aboveground CO2-equivalent stocks, whereas in silvopastoral systems only five species explained a similar proportion. Dominant taxa such as Cordia alliodora, Inga edulis, Jacaranda copaia, Piptocoma discolor, and Piptadenia pteroclada illustrate a process of biocultural species filtering, whereby trees providing food, timber, shade, and cultural value are selectively retained while sustaining significant carbon stocks. These findings demonstrate that tree-based productive systems function as biocultural productive landscapes that conserve carbon, biodiversity, and livelihoods beyond forest boundaries. We argue for their formal inclusion, particularly traditional silvopastoral systems, within climate finance mechanisms, nationally determined contributions (NDCs), and biocultural heritage frameworks, alongside forest conservation strategies.

1. Introduction

Tropical landscapes have become increasingly characterized by mosaics in which old-growth forests coexist with human-managed production systems. Across the global tropics, the expansion of pastures and commodity crops has fragmented primary forests, driving biodiversity loss, altered ecosystem functions, and depleted carbon stocks [1,2,3,4]. However, a growing body of evidence shows that tree-based production systems particularly agroforestry and silvopastoral systems retain key structural and functional attributes of forests. These systems provide significant climate mitigation and biodiversity co-benefits while sustaining local livelihoods and contributing to multiple Sustainable Development Goals (SDGs) [5,6,7]. As smallholder-managed agroforestry and silvopasture increasingly occupy large portions of tropical landscapes, they create multifunctional mosaics that challenge conventional models that assume a rigid separation between conservation and production spaces.
In many tropical smallholder systems, tree cover is not a passive remnant of past forest clearance but the result of intentional management decisions. Local farmers, drawing on long-standing ecological knowledge, retained and planted multifunctional species that supported shade-tolerant crops, providing fruit, timber, fodder, and medicine, and sustained habitat diversity. These practices reflect a deep history of coexistence between people and forests, in which trees formed the ecological and cultural backbone of productive landscapes. As market integration expanded, producers have adapted rather than abandoned their forest-informed systems, maintaining their livelihoods under increasing market pressures while preserving the biocultural foundations of production. They have integrated crops such as cacao into tree-rich agroforestry and silvopastoral mosaics that maintain high biodiversity and aboveground carbon storage [8,9]. This adaptive continuity underscores livelihood resilience but also illustrates how market-linked traditional systems have continued to operate as biocultural productive landscapes. Unlike generic agroforestry systems or conventional silvopastoral practices, which often retain trees opportunistically or as residual elements of forest conversion, existing frameworks, such as Working Landscapes [10] and Biocultural Landscapes [11], only partially capture the ecological and cultural dynamics of tree-based productive systems. While the former emphasizes multifunctionality in production areas and the latter highlights the co-evolution of cultural identity and ecological processes, neither explicitly integrates measurable ecological outcomes—such as carbon retention and species richness—with culturally guided species selection under market conditions.
To address this gap, we introduce the concept of Biocultural Productive Landscapes (BPLs) as an operational framework that links culturally mediated tree management with quantifiable ecological performance. BPLs are characterized by the intentional selection and long-term stewardship of multifunctional tree species, shaped by Traditional Ecological Knowledge, cultural values, and co-evolved human–forest relationships, while remaining actively integrated into market-oriented production systems [10,11,12,13,14,15].
We hypothesize that tree-based traditional production systems embedded within the Andean–Amazon landscape function as biocultural carbon and biodiversity connectors at the landscape scale, retaining substantial proportions of forest carbon stocks beyond forest boundaries, that traditional silvopastoral systems retain carbon stocks comparable to cacao-based agroforestry systems, and that carbon storage in these productive systems is disproportionately concentrated in a limited number of multifunctional tree species intentionally selected and retained through biocultural management.
The transition zone between the Andes and Amazon in Ecuador provides a suitable setting for examining biocultural productive systems under active land-use transformation. This study focuses on the canton of Arosemena Tola as a site-level case study situated within the Tropical Andes biodiversity hotspot [16,17,18] and the transition area of the UNESCO-recognized Sumaco Biosphere Reserve [19]. The canton encompasses traditional Amazonian Chakra agroforestry, tree-rich silvopastoral systems, and remnant old-growth forests within a contiguous landscape mosaic, enabling direct structural comparison among contrasting land uses under comparable climatic and edaphic conditions.
The area is characterized by active market integration through cacao commercialization and livestock production, creating sustained interactions between culturally rooted management practices and contemporary economic drivers. This combination of ecological heterogeneity, land-use continuity, and market exposure provides an analytically appropriate context for assessing structural and carbon dynamics across tree-based productive systems within a defined territorial unit.
Among these, the traditional Amazonian Chakra agroforestry system (AFS)—officially designated as a Globally Important Agricultural Heritage System (GIAHS) by FAO in 2023—embodies a biocultural strategy that has sustained food production, ecological functions, and livelihood resilience in Kichwa communities for generations [20,21]. Complementing this system are traditional silvopastoral systems (SPS), where native trees are intentionally retained for timber, shade, fruit, and fodder, creating diversified livestock landscapes with significant ecological functionality [22]. Together, the traditional Chakra AFS and SPS form a biocultural landscape mosaic, operating as biocultural productive landscapes in practice, in which forest remnants and productive land uses remain ecologically intertwined. Despite ongoing land-use change and forest loss, local strategies of selective tree retention have preserved key ecological legacies—maintaining microclimate regulation, species dispersal pathways, and carbon connectivity across increasingly fragmented terrains [10,23].
Although Ecuador’s updated NDC 2020–2050 [24] and its National Adaptation Plan 2023–2027 [25] recognize agroforestry within broader agricultural and adaptation sectors, traditional tree-based systems, such as the Amazonian Chakra, are only indirectly framed within broader productive or resilience-oriented measures rather than explicitly positioned as integrated carbon–biodiversity strategies. Similarly, tree-rich silvopastoral systems receive limited explicit recognition as climate mitigation or biodiversity conservation instruments within national policy architecture. While recent studies have highlighted the multifunctional benefits of agroforestry and silvopasture, empirical evidence from tropical contexts like Ecuador has been limited [26]. This pattern reflects a broader global trend in which agroforestry is increasingly acknowledged in climate discourse, yet still underrepresented as a measurable nature-based solution within mitigation accounting frameworks [23,27,28].
A growing body of research has quantified carbon stocks in tropical agroforestry and silvopastoral systems [29,30]. However, most studies have assessed these land uses separately or focused primarily on biophysical metrics. Few have simultaneously integrated structural carbon retention, tree biodiversity, and biocultural management within a unified landscape framework. Comparative empirical evidence from the Andean–Amazon transition zone remains limited, particularly regarding the structural role of traditional silvopastoral systems alongside cacao-based agroforestry [31,32]. This gap constrains a comprehensive understanding of how tree-based productive systems collectively operate within biocultural landscapes and contribute to climate mitigation beyond forest boundaries [10,27].
Accordingly, this study had three objectives: (i) quantify and compare tree diversity, structure, and carbon stocks across apparently non-disturbed old-growth forests, traditional cacao-based agroforestry systems (Amazonian Chakra), and tree-rich silvopastoral systems; (ii) to examine how tree richness, size distribution, and structural complexity influence carbon storage; and (iii) to assess how these tree-based systems contribute to maintaining ecological structure and carbon connectivity within a fragmented Andean–Amazonian landscape.
Building on this premise, the next section develops the theoretical underpinnings of this study, integrating perspectives from multifunctional and biocultural landscape frameworks to establish the conceptual basis for the Biocultural Productive Landscape (BPL) approach, explicitly linking it to market-connected traditional systems.

2. Theoretical Framework

2.1. Multifunctional and Biocultural Tree-Based Landscapes

In tropical regions, forests increasingly coexist with tree-based production systems managed by Indigenous and smallholder communities. Agroforestry and silvopastoral systems, when culturally maintained, retain substantial ecological functionality—preserving tree diversity, biomass, and carbon stocks comparable to secondary forests [13,29]. These multifunctional landscapes provide ecosystem services, such as microclimate regulation, soil fertility, and habitat continuity, while supporting rural livelihoods and contributing to several SDGs [33,34]. In this sense, they blur the traditional divide between conservation and production by demonstrating that well-managed agricultural mosaics can simultaneously deliver ecological and economic outcomes [10].
The persistence of trees within these systems is not an ecological coincidence but the result of culturally guided management. Traditional Ecological Knowledge (TEK) informs species selection, shade management, and regeneration dynamics [10,11,12,35]. Farmers retain or plant multifunctional native species that provide shade, fruit, fodder, timber, and medicinal resources, creating structurally complex canopies that sustain biodiversity and production [15,36]. In the Andean–Amazon region, Indigenous and mestizo communities have long lived within and alongside forests, developing livelihood strategies based on coexistence rather than deforestation [37]. As market integration has expanded, they have adapted these biocultural logics rather than replacing them, incorporating shade-tolerant crops such as cacao into tree-rich systems that maintain high carbon storage and species richness [37,38]. These dynamics reveal that many Amazonian productive landscapes are, in essence, forest-informed systems—landscapes shaped by stewardship that sustain ecological processes while meeting subsistence and commercial needs [29].
Recognizing this intentional management reframes these territories as vital elements for biodiversity conservation and climate mitigation. Their persistence underscores the need to view smallholder-managed systems not as transitional forms between forest and agriculture, but as enduring, multifunctional landscapes integrating ecology, culture, and production [35,39,40].

2.2. The Biocultural Productive Landscape Concept

Building on these insights, this study advances the concept of Biocultural Productive Landscapes (BPLs), tree-based territorial systems where ecological processes, cultural practices, subsistence production, and market-oriented activities coexist in mutually reinforcing ways. BPLs emerge from long-term human–forest relationships that maintain ecological integrity through culturally mediated management. They integrate ecological multifunctionality with TEK-based stewardship, providing a framework to understand how local communities sustain biodiversity, carbon, and livelihoods within productive mosaics [36,39,41].
In this study, the concept of BPLs is applied as an integrative analytical framework that links three interrelated dimensions: (i) structural carbon retention, (ii) partial maintenance of tree species richness and functional diversity, and (iii) continuity of management practices grounded in Traditional Ecological Knowledge within contemporary production systems [42].
Unlike Working Landscapes, which emphasize multifunctionality in production areas [10], and Biocultural Landscapes, which foreground long-term cultural–ecological co-evolution [11], the BPL framework explicitly incorporates measurable ecological indicators alongside socio-economic dynamics. This integration is particularly relevant in climate policy contexts, such as NDC and REDD+ frameworks, which have historically centered mitigation efforts on forest conservation and deforestation reduction while granting comparatively less explicit attention to structurally complex tree-based production systems [27,28].
To situate this contribution within existing scholarship, Table 1 summarizes the main frameworks underpinning the BPL approach. While working landscapes highlight multifunctionality, biocultural landscapes emphasize the co-evolution of nature and culture through TEK, cultural landscape stewardship focuses on participatory heritage-based management, and Earth stewardship promotes socio-ecological transitions. The BPL framework expands these perspectives by empirically linking culture, carbon retention, and market adaptation within tropical tree-based systems—an integrated vision further elaborated in Box 1, which formalizes the conceptual definition introduced in this study.
Table 1 outlines the conceptual foundations informing the BPL framework; however, its contribution is not only synthetic but also operational, as formalized in Box 1. Whereas Working Landscapes primarily articulate multifunctionality at the landscape scale [10], and Biocultural Landscapes emphasize cultural–ecological co-evolution mediated by TEK [11], BPL approach advances these perspectives by explicitly integrating measurable ecological retention metrics within productive systems alongside management practices grounded in Traditional Ecological Knowledge [27,42]. This operationalization is reflected in the comparative assessment of forest-referenced carbon stocks, tree species richness, and species-use composition across land-use types. By embedding culturally informed management decisions within a quantifiable structural framework, BPLs become analytically distinguishable as socio-ecological systems characterized by measurable ecological performance.
Box 1. Definition of a Biocultural Productive Landscape.
We define Biocultural Productive Landscapes (BPLs) as territorial systems where ecological processes, cultural practices, and Traditional Ecological Knowledge (TEK) interact with subsistence and market-oriented production in mutually reinforcing ways. Unlike strictly protected forests or conventional monocultures, BPLs maintain substantial tree cover, species richness, and aboveground carbon stocks while sustaining culturally embedded livelihood strategies.
Tree retention and enrichment in BPLs are deliberate outcomes of local decision-making, shaped by TEK and long-standing relationships with the forest. Communities selectively maintain multifunctional native species that support shade-tolerant crops, provide resources for human and animal use, and reinforce cultural identity. These practices reflect adaptive continuity: as markets evolve, producers adjust rather than replace traditional forest-based management, resulting in productive systems that remain ecologically rich and carbon-dense.
Conceptually, BPLs integrate and extend two major perspectives: (i) biocultural landscapes, emphasizing long-term human–nature co-evolution and the role of TEK in shaping ecosystem patterns [11] and (ii) Working landscapes, recognizing multifunctional production spaces that conserve ecosystem processes while generating economic value [10,44]. Together, these frameworks converge in the BPL concept, which positions forest-informed production systems as central to sustainable rural futures in the Andean–Amazon region.

3. Materials and Methods

3.1. Study Area

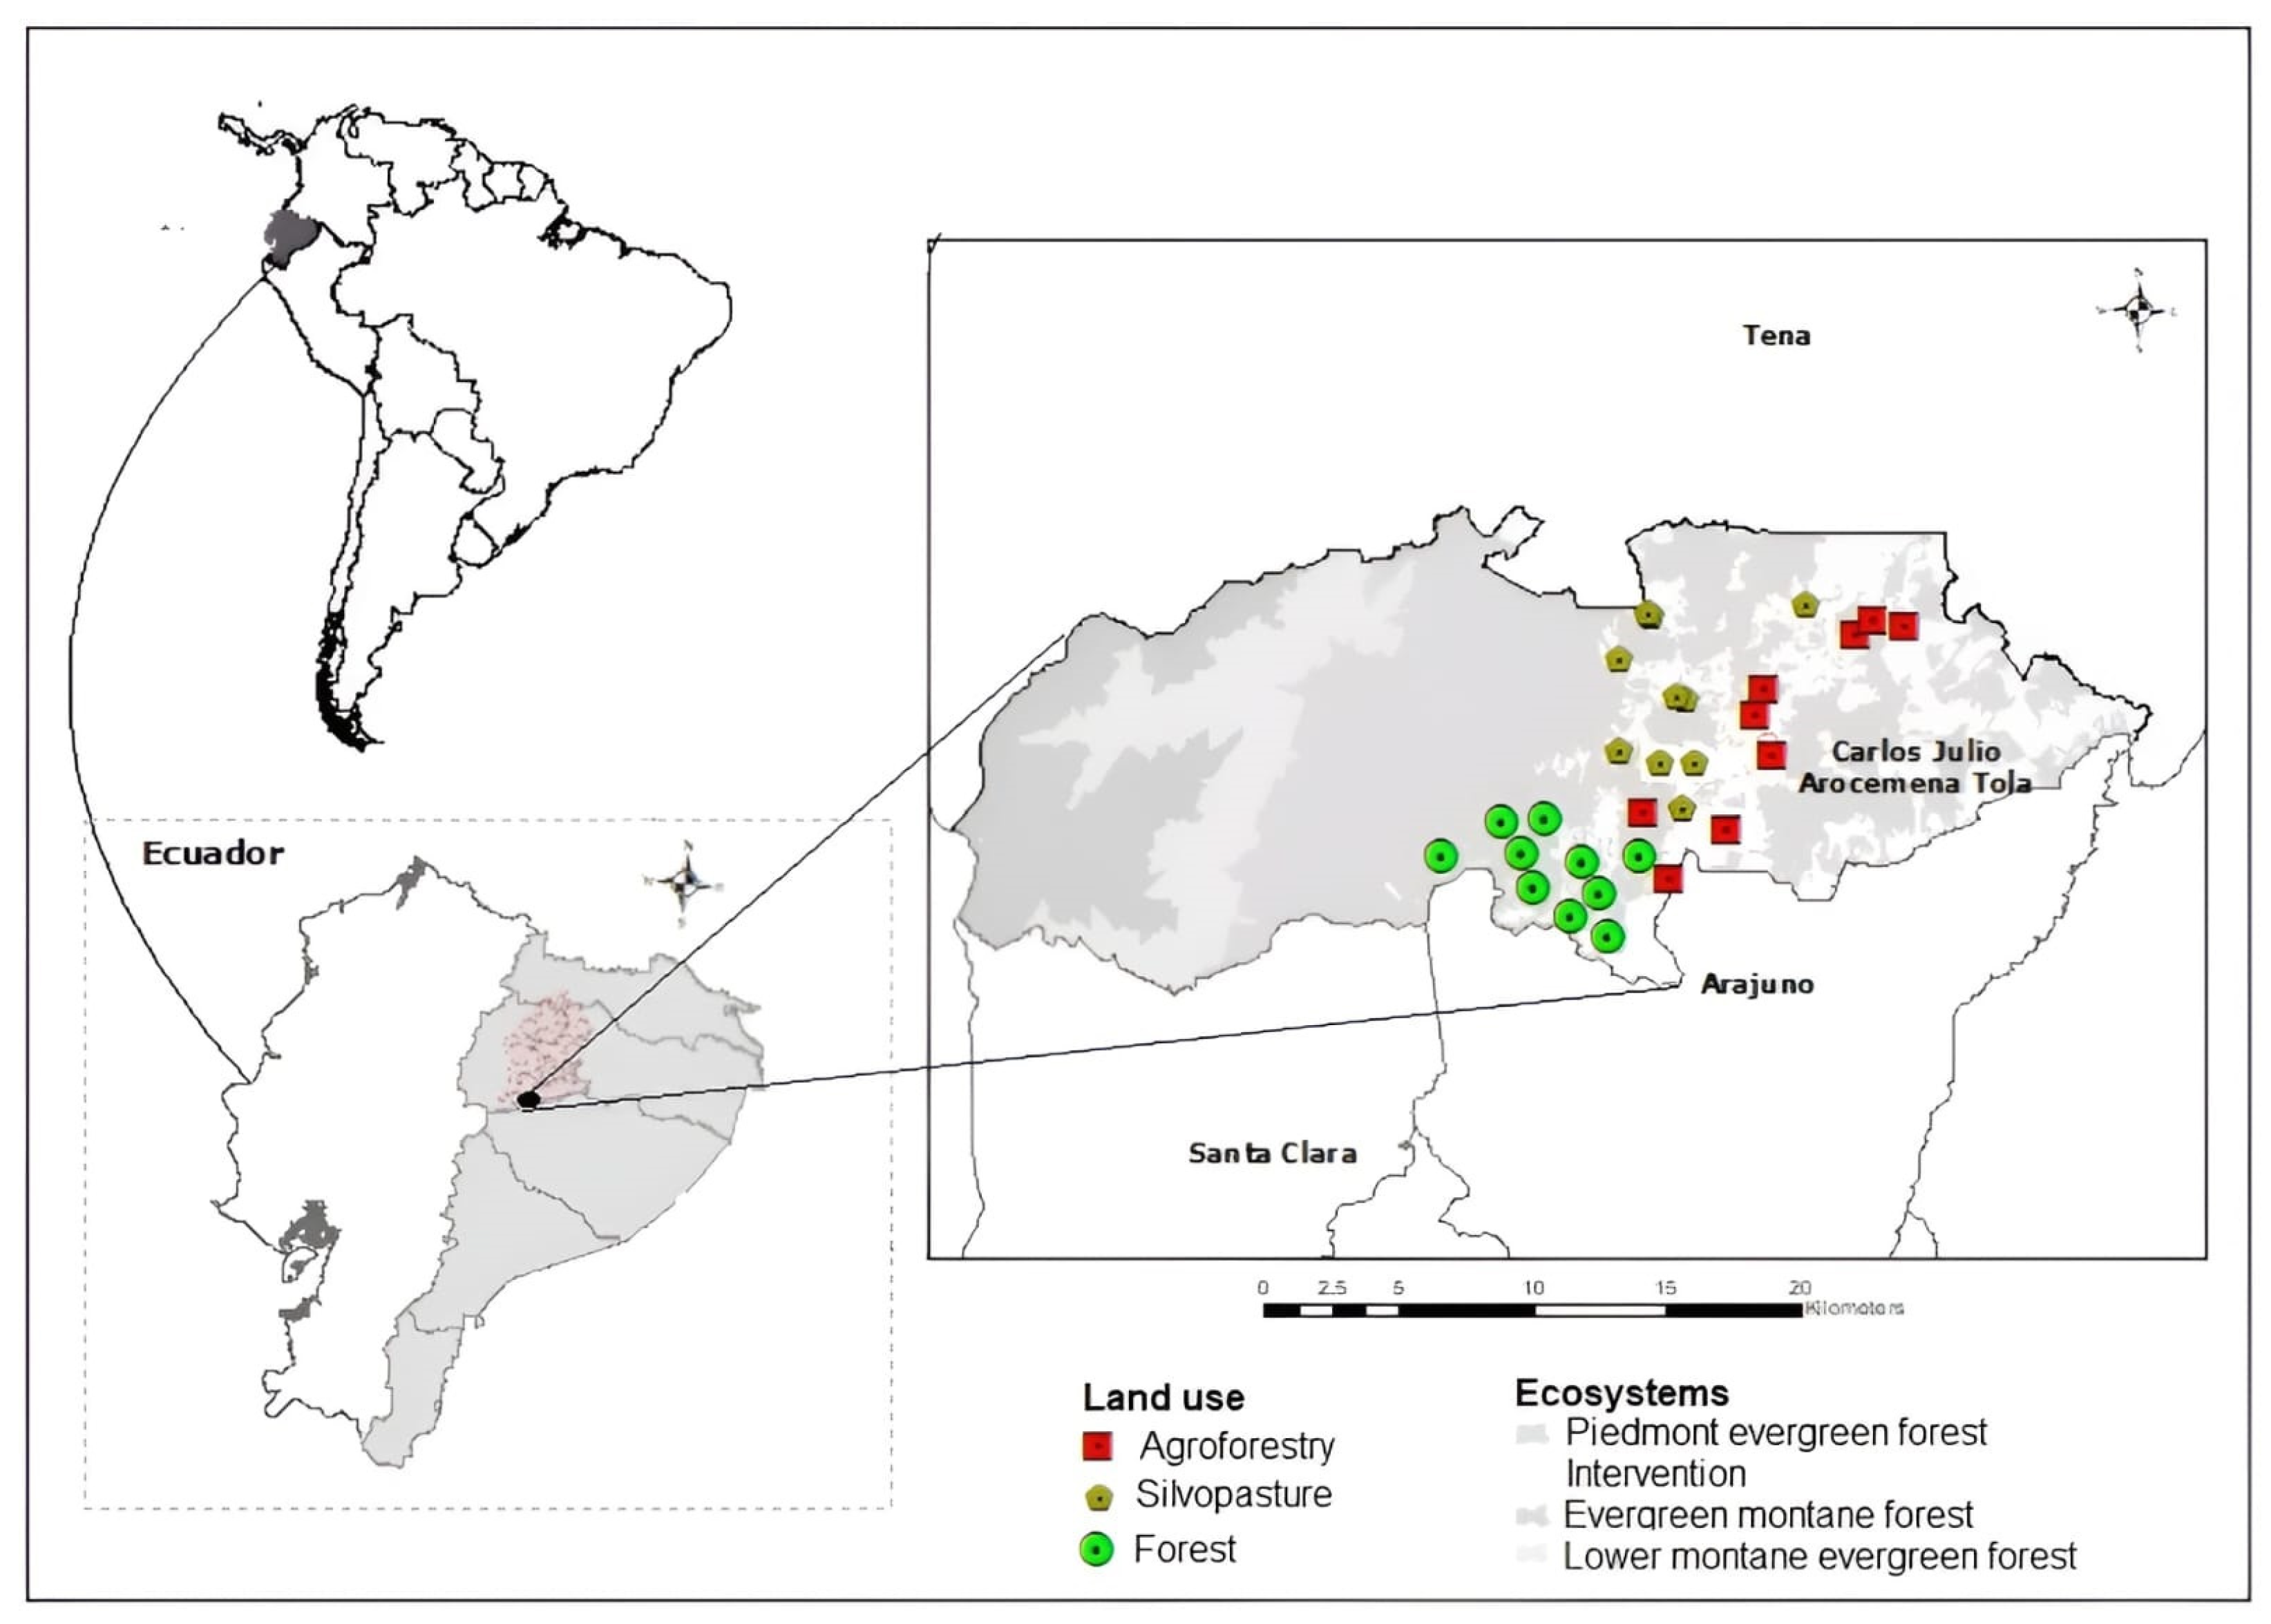
This study was conducted in the Canton Carlos Julio Arosemena Tola, in the province of Napo, Ecuador, within the lower montane zone (400–800 m.a.s.l.) of the Sumaco Biosphere Reserve (SBR). This territory lies within the Western Amazon biodiversity hotspot [16,18], where a mosaic of land uses includes remnant primary forests, traditional cacao-based agroforestry systems, and tree-rich silvopasture (Figure 1). These systems were established approximately five decades ago and are predominantly managed by smallholder households engaged in mixed cacao cultivation and cattle production, reflecting a long-standing biocultural interaction between livelihoods and forest structure [15,41]. Such a configuration aligns with the “matrix” perspective proposed by Perfecto, Vandermeer and Wright [13], in which biodiversity and ecosystem functions are not restricted to protected forests but emerge across multifunctional agricultural landscapes where tree cover and ecological connectivity are maintained.

3.2. Bioclimatic Characteristics

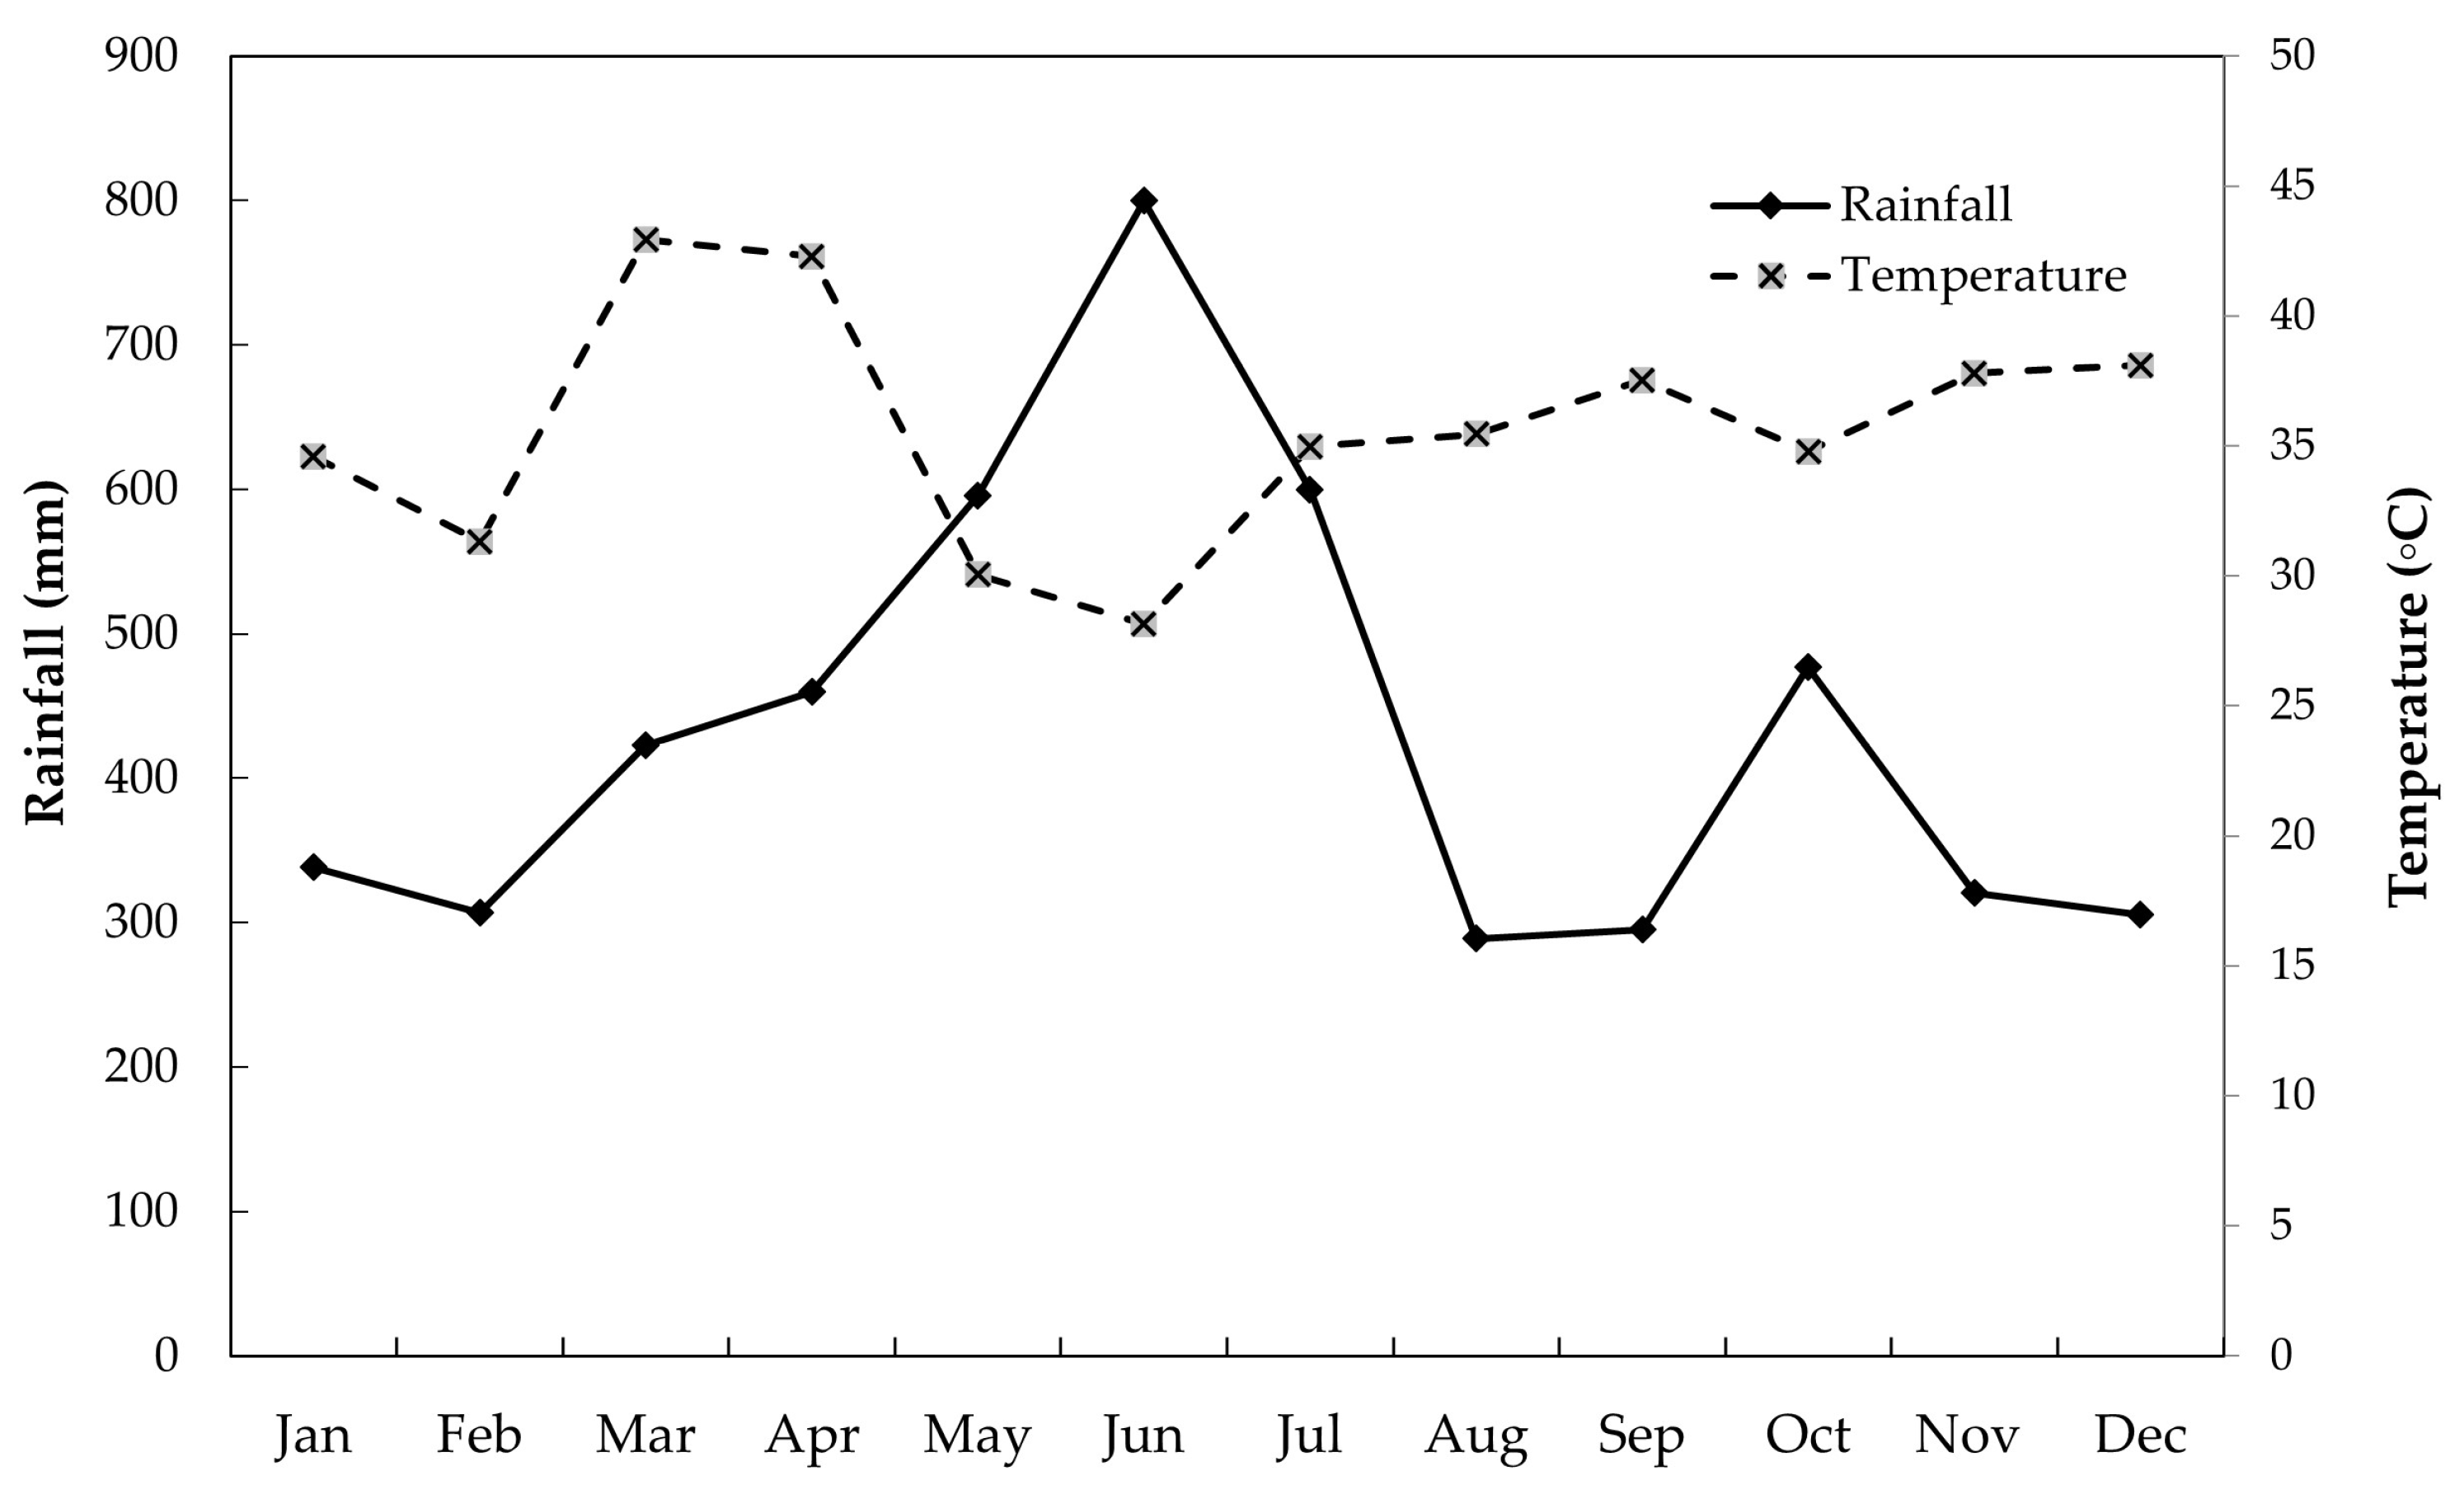
The study area exhibits a humid tropical climate with marked seasonality in rainfall but relatively stable temperatures throughout the year (Figure 2). Mean monthly precipitation ranges from ~280 mm in the dryest months (August–September) to over 750 mm in the wettest period (June), contributing to an annual total exceeding 5000 mm. Temperatures remain high year-round, fluctuating between 30 °C and 40 °C, with a mean annual value of approximately 35.7 °C. This combination of high rainfall and warm conditions reflects the humid premontane Amazonian environment typical of the low-elevation belt (400–800 m.a.s.l.) of Arosemena Tola [45].

3.3. Field Methods

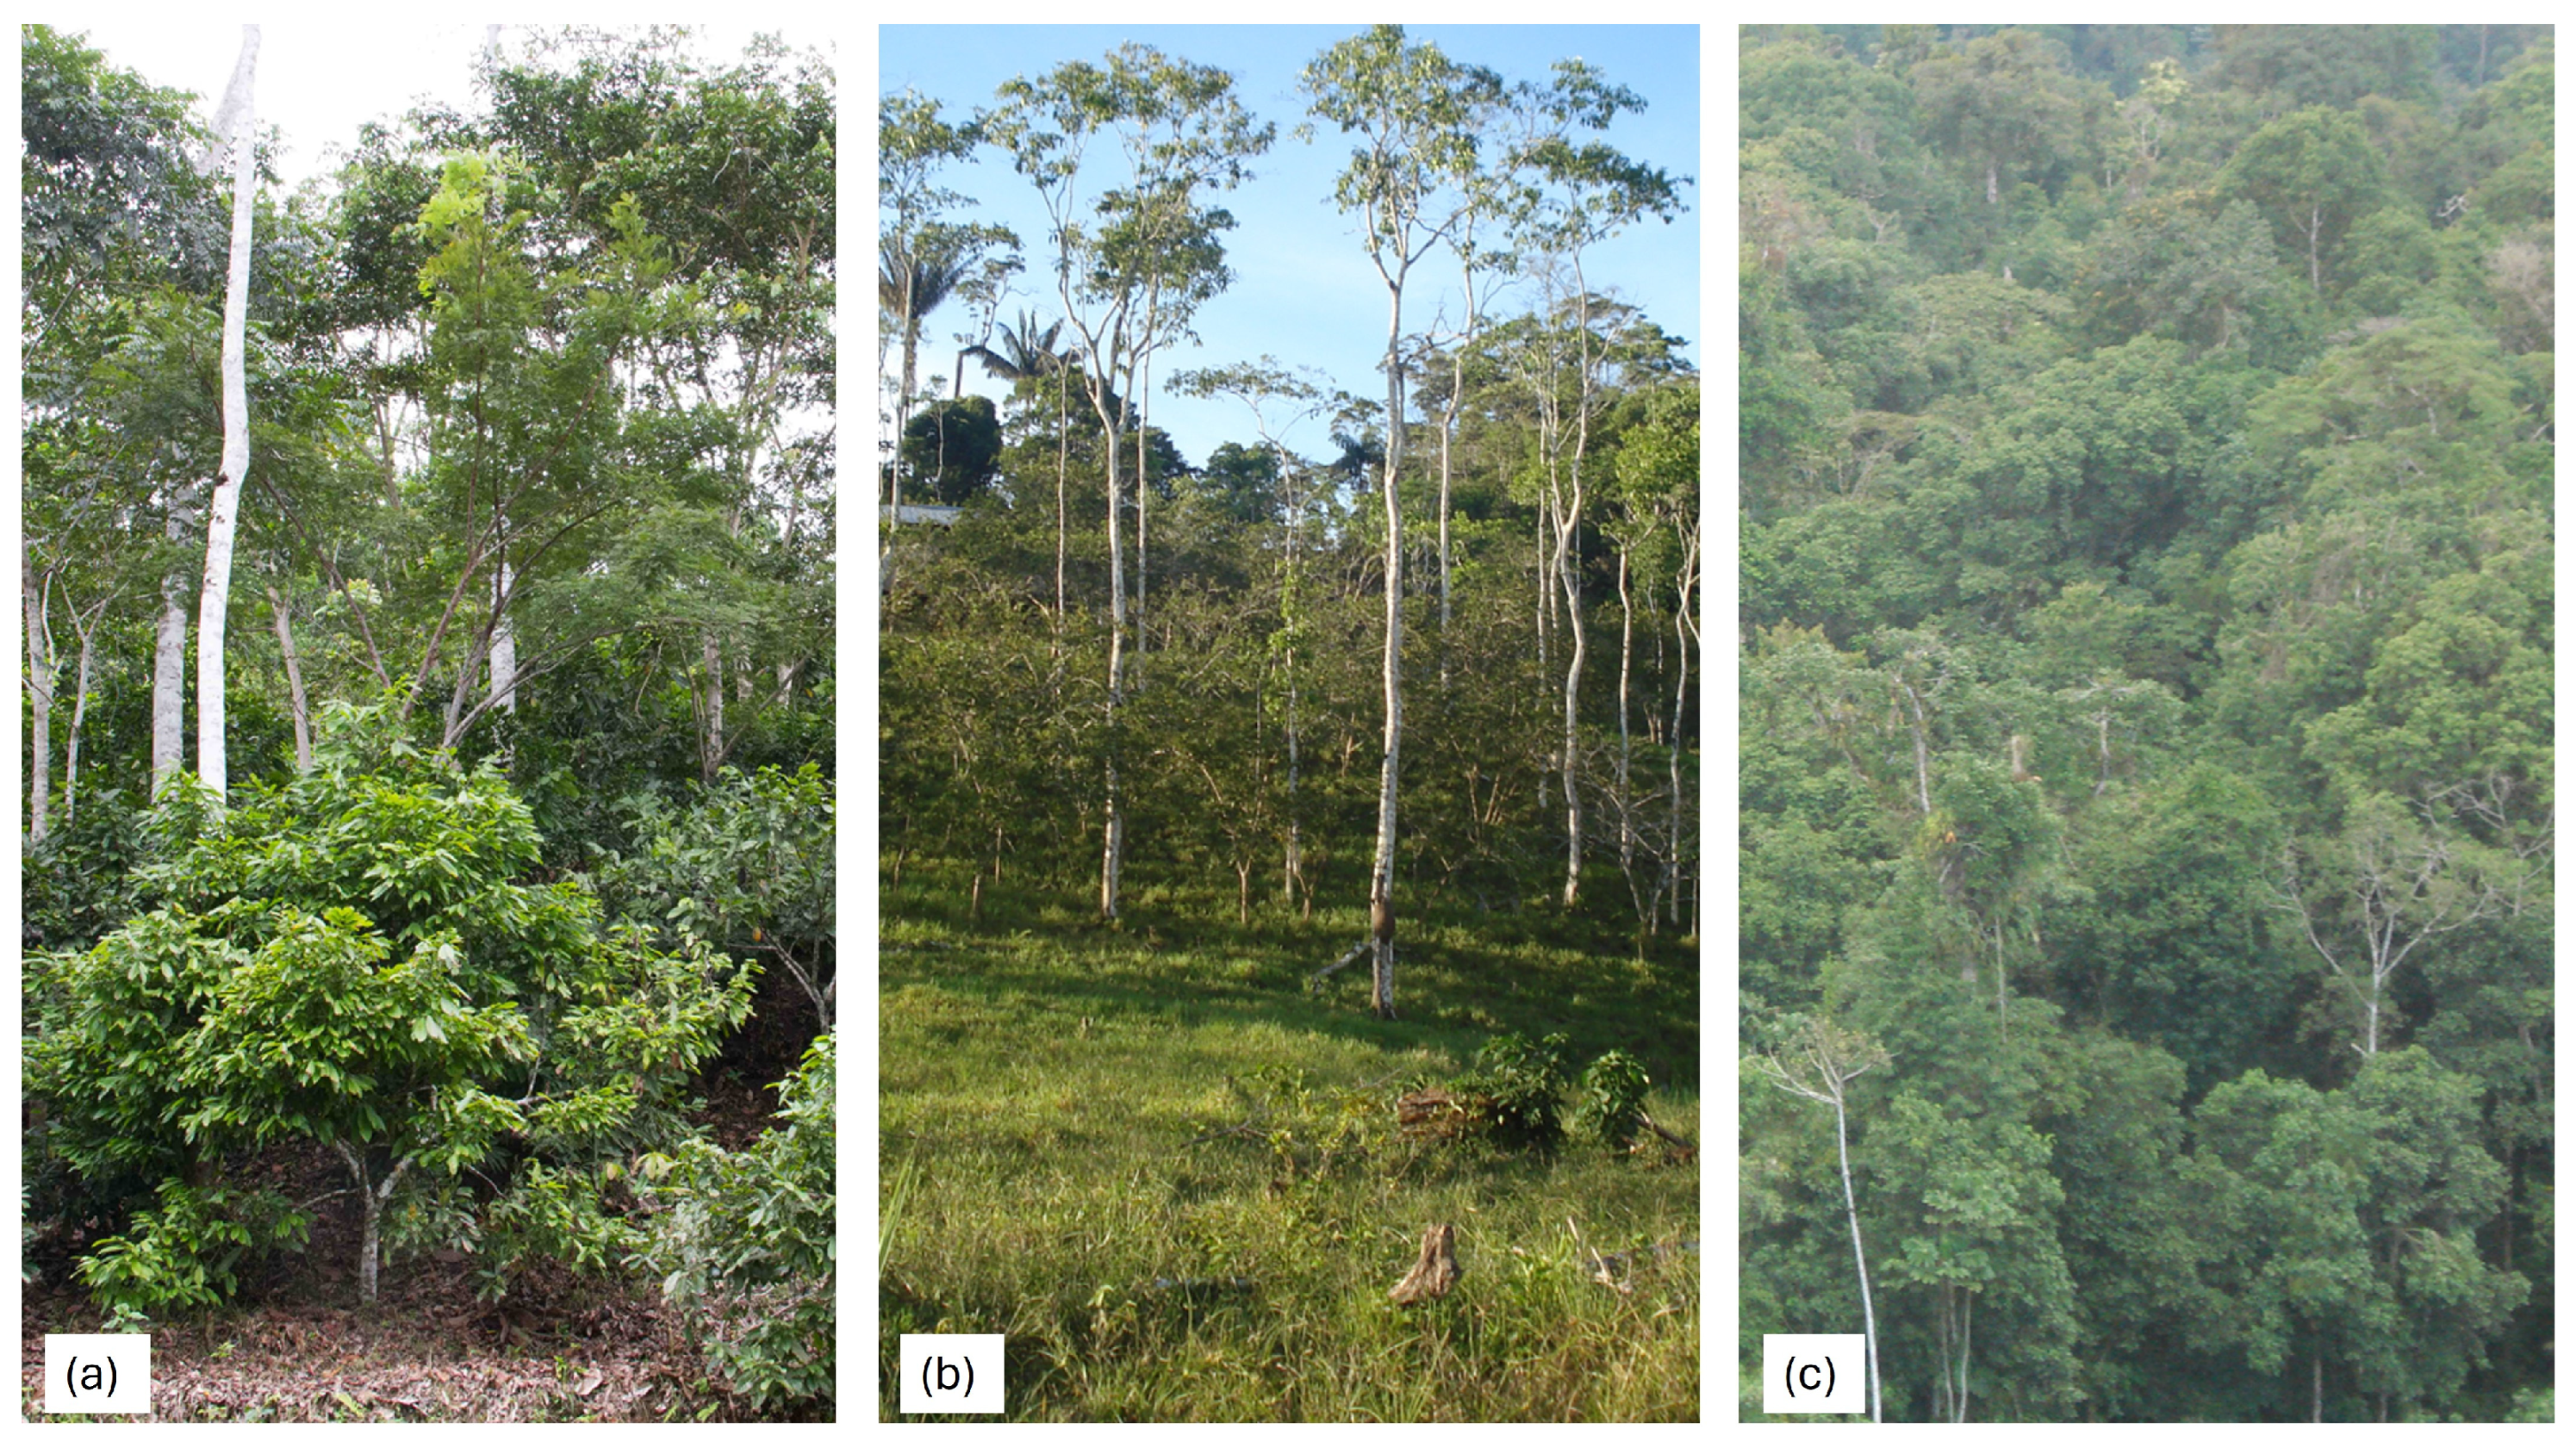
A total of 28 temporary sampling plots were established across the three land-use systems evaluated (Figure 3), following a stratified design that accounted for land-use categories and environmental gradients, consistent with the agroecological matrix perspective applied in tropical multifunctional landscapes [13]. In agroforestry systems (AFS), nine square plots of 1600 m2 (40 × 40 m) were installed to capture the heterogeneous, multi-strata tree arrangement typical of cacao-based systems. In silvopastoral systems (SPS), nine circular plots of 2826 m2 (30 m radius) were used to adequately represent the scattered distribution of remnant and managed trees in pasture matrices. In forest sites, ten rectangular plots of 1000 m2 (10 × 100 m) were established in selectively logged old-growth forest stands. The use of different plot sizes and shapes was justified by logistical considerations and the need to capture the characteristic spatial distribution of trees in each system, following methodological recommendations for tropical forest, agroforestry, and silvopastoral assessments [30,46,47]. All plots were georeferenced and inventoried following standard tropical forest sampling protocols.
The use of different plot sizes and geometries responded to the distinct spatial configuration of trees within each land-use system, a common approach in comparative studies of tropical forests and agroforestry mosaics where tree density and spatial dispersion differ substantially among matrices [13,29,30]. While perimeter–area relationships vary among plot shapes, all structural and biomass variables were standardized to a per-hectare basis before analysis, following established practice in tropical forest inventory and carbon assessment studies [48,49]. This ensured that observed differences reflect structural characteristics of land-use systems rather than bias of plot geometry. To reduce edge effects, trees were included only when at least 50% of the stem base fell within the plot boundary, following standard forest inventory criteria. Sampling was conducted at the household level, resulting in spatially dispersed plots across independently managed landholdings (Figure 1), which reduced the likelihood of spatial autocorrelation. Visibly anomalous or recently disturbed patches were excluded to avoid distortion of structural estimates. Similar multi-design sampling approaches have been widely applied in studies comparing tropical forests, agroforestry, and silvopastoral systems, where tree spatial patterns, density, and canopy structure differ markedly across land uses [13,29,30]. To enable robust comparisons, all structural, diversity, biomass, and carbon variables were standardized per hectare before statistical analyses, following established practices in assessments of tropical forest- and tree-based systems [48,49]. The goal of this standardization was to minimize potential bias associated with plot size or shape and to ensure that observed differences among land-use systems reflect underlying ecological patterns rather than sampling design effects. Although differences in plot geometry may introduce some variation in edge-related effects, the standardized sampling area and comparative (rather than spatially explicit) objective of this study make it unlikely that such variance would systematically alter relative structural contrasts among systems.
This study was designed as a site-level comparative structural assessment rather than a spatially explicit landscape-scale inventory; accordingly, interpretations are bounded to this analytical and spatial scope.
All live trees with diameter at breast height (DBH) ≥ 10 cm were measured and taxonomically identified by local specialists, and voucher specimens were collected for verification in the ECUAMZ herbarium (Universidad Estatal Amazónica, Ecuador) when required, following established protocols for floristic surveys in Amazonian tree-based systems [50]. Basal area (m2 ha−1) was calculated as a structural proxy using the standard formula:
B a s a l   a r e a = π × D B H 2 2   scaled   by   plot   area
where DBH = Diameter at breast height (m).
Aboveground biomass (AGB) was estimated for all trees with DBH ≥ 10 cm using the moist tropical forest allometric model proposed by Chave et al. [51]:
A G B = ρ   e x p 1.499 + 2.148   l n ( D B H ) + 0.207 ( l n   D B H ) ) 2 0.0281 ( l n ( D B H ) ) 3 )
where AGB is expressed in kilograms of dry mass, ρ is wood density (g cm−3), and DBH is the diameter at breast height (cm). Species-specific wood density values were assigned from neotropical databases [50,52,53]. When species-level data were unavailable, a mean wood density of 0.47 g cm−3 was used for agroforestry and silvopastoral systems, consistent with recommended averages for tropical secondary forests and managed tree-based systems [30,48], In contrast, forest plots were assigned a higher mean wood density (0.63 g cm−3), reflecting the predominance of mature, late-successional taxa typical of old-growth Amazonian forests [54]. Biomass and carbon estimates in tropical systems are inherently associated with uncertainty arising from allometric model selection, wood density assignments, plot-level variability, and the use of generalized root–shoot ratios [48,51,55]. While species-specific wood densities were applied when available, mean values and standardized coefficients were used where necessary to ensure methodological consistency across land-use types. Such approaches are widely adopted in comparative tropical biomass studies when the objective is structural comparison rather than formal greenhouse gas accounting [27,29]. Because identical allometric equations and carbon conversion factors were applied across all systems, potential systematic biases would affect land uses uniformly, preserving the validity of relative comparisons within the studied mosaic. Nevertheless, absolute carbon magnitudes should be interpreted within the analytical framework and coefficient assumptions employed.
Belowground biomass (BGB) was estimated as a proportion of aboveground biomass (AGB), using a standard coefficient of 0.30 widely applied in comparative tropical studies and consistent with root: shoot ratios reported in the literature and IPCC methodologies for tropical forests when direct measurements are unavailable [55,56,57]. This approach ensured methodological consistency across land-use systems. However, root-to-shoot ratios may vary according to ecological conditions, functional composition, and management practices; therefore, system-specific BGB estimates could further refine future assessments. Carbon stocks were calculated by multiplying above- and belowground biomass by a carbon concentration factor of 0.47 [58]. The carbon estimation approach was applied to ensure methodological consistency and was not intended for formal climate accounting.
Before statistical analyses, assumptions of normality and homogeneity of variances were evaluated using Shapiro–Wilk and Levene tests, respectively. Logarithmic transformations were applied when necessary, following analytical procedures commonly employed in studies of tropical forest structure and carbon dynamics [29,30]. Differences among land-use systems were assessed using one-way ANOVA, followed by Tukey post hoc tests. All statistical analyses were performed in SPSS v.22 (IBM Corp., Armonk, NY, USA). In addition to significance testing, standardized effect sizes (Cohen’s d) and 95% confidence intervals (95% CI) were calculated to quantify the magnitude of differences in total tree carbon stocks among land-use systems, following conventional benchmarks for interpretation [59,60]. Reporting effect sizes allows assessment of ecological relevance beyond p-values and facilitates comparison across studies.

4. Results

4.1. Tree Diversity and Structural Attributes Across Land Uses

Tree diversity and forest structure showed marked variation along the agroforestry–silvopastoral–forest gradient in Arosemena Tola (Table 2). Tree density differed significantly among systems (p < 0.001), with forests exhibiting more than three times the number of individuals per hectare (626 ± 117 ind ha−1) compared to agroforestry (177 ± 105) and silvopastoral systems (194 ± 112). This pattern reflects the higher canopy closure and regeneration potential maintained in forest stands. Importantly, agroforestry and silvopastoral systems retained approximately 28–30% of forest tree density, indicating that a substantial fraction of forest structural attributes persists within the agricultural matrix.
Mean diameter at breast height (DBH) ranged from 19.2 cm in agroforestry to 22.0 cm in forest plots, but differences were not statistically significant (p > 0.05), suggesting that a few large remnant trees persist in productive systems, compensating for lower stem densities. The persistence of these large individuals (DBH > 40 cm), despite land-use change, contributes disproportionately to structural complexity and carbon storage, acting as “structural anchors” for aboveground biomass and canopy structure within the productive landscape. Trees with DBH > 40 cm represented around 9% of total individuals in forest plots, compared to 3% in agroforestry systems and 6% in silvopastoral systems. Despite their lower relative abundance in managed systems, these large individuals contributed disproportionately to aboveground carbon stocks, accounting for approximately 55% of total tree carbon in forests, 17% in agroforestry, and 45% in silvopastoral systems. This concentration of biomass within a limited number of large stems supports their role as structural carbon anchors within each land-use type. In contrast, basal area differed strongly among land uses (p < 0.001), averaging 30.8 ± 9.2 m2 ha−1 in forests, compared to only 5.9 ± 4.3 in agroforestry and 7.8 ± 4.4 in silvopasture. This represents a 74–81% reduction in standing basal area relative to forests, reinforcing the structural simplification outside the forest matrix.
Tree diversity followed similar trends. Species richness (S), family richness, and Shannon (H′) and Simpson (1–D) indices were significantly higher in forests (H′ = 2.90 ± 0.23) than in agroforestry (H′ = 1.22 ± 0.44) or silvopastoral systems (H′ = 1.45 ± 0.35; p < 0.001). Agroforestry and silvopastoral systems retained between 22 and 29% of forest species richness, demonstrating partial but meaningful conservation of native flora within productive land uses. While productive systems retained subsets of native and multipurpose species, their reduced richness and structural complexity reveal partial erosion of floristic diversity relative to forest conditions. However, the presence of overlapping species among the three systems (e.g., Cordia alliodora, Inga spp., Jacaranda copaia) suggests ecological continuity and supports the role of productive systems as functional connectors within the landscape mosaic.

4.2. Above- and Below-Ground Biomass and Carbon Stocks

Biomass and carbon stocks differed significantly among land uses (p < 0.001), showing a clear gradient from forest to silvopastoral and agroforestry systems (Table 3). Forests exhibited the highest above-ground biomass (AGB) values, averaging 283.9 ± 103.2 Mg ha−1, which was more than three times greater than in silvopastoral systems (81.4 ± 48.2 Mg ha−1) and over six times higher than in agroforestry plots (45.9 ± 33.6 Mg ha−1). The same pattern was observed for above-ground carbon (AGC), with forests storing 133.4 ± 48.5 Mg C ha−1 compared to 37.9 ± 26.7 in silvopasture and 21.6 ± 15.8 in agroforestry. This gradient indicates a strong decline in biomass and carbon storage with increasing land-use intensity.
Below-ground biomass (BGB) followed similar trends, with significantly higher values in forests (85.2 ± 30.9 Mg ha−1) than in silvopastoral (24.4 ± 14.5 Mg ha−1) and agroforestry systems (11.7 ± 10.3 Mg ha−1). This parallel response suggests that root systems contribute consistently to total carbon stocks across land-use types. Correspondingly, total tree biomass averaged 369.0 ± 134.1 Mg ha−1 in forests, 105.8 ± 65.6 in silvopasture, and 59.7 ± 43.1 in agroforestry (p < 0.001).
When expressed as total tree carbon, forests contained 173.4 ± 63.0 Mg C ha−1 more than triple the stocks found in productive systems (49.3 ± 29.5 in SPS; 28.1 ± 20.5 in AFS). This pattern suggests a pronounced reduction in carbon storage along the land-use gradient, although the persistence of remnant trees in agroforestry and silvopastoral systems contributes meaningfully to landscape-level carbon retention. In addition, a positive association was observed between basal area and carbon stocks across land uses, indicating that structural attributes, particularly the presence of large trees, play a central role in explaining carbon retention patterns.
In addition to statistical significance values, effect sizes (Cohen’s d) and 95% confidence intervals (95% CI) were estimated to assess the practical magnitude of differences in total tree carbon among production systems. The mean difference between silvopastoral systems (SPS) and agroforestry systems (AFS) was Δ = 21.2 Mg C ha−1 (SPS > AFS), with a 95% CI of [−2.3, 44.7] Mg C ha−1. The standardized effect size was d = 0.83, corresponding to a moderate-to-large effect according to conventional benchmarks. Although the confidence interval slightly overlaps zero, these results indicate that the magnitude of the difference between AFS and SPS is intermediate relative to the intrinsic variability observed within both systems.
In contrast, the difference between forest and agroforestry systems was substantially greater (Δ = 145.4 Mg C ha−1; 95% CI [104.1, 186.7] Mg C ha−1; d = 3.03), representing a very large and consistent effect. These findings confirm that the sampling design has sufficient power to detect substantial structural divergences when present, whereas the comparison between AFS and SPS reflects partially convergent magnitudes within the evaluated landscape mosaic.
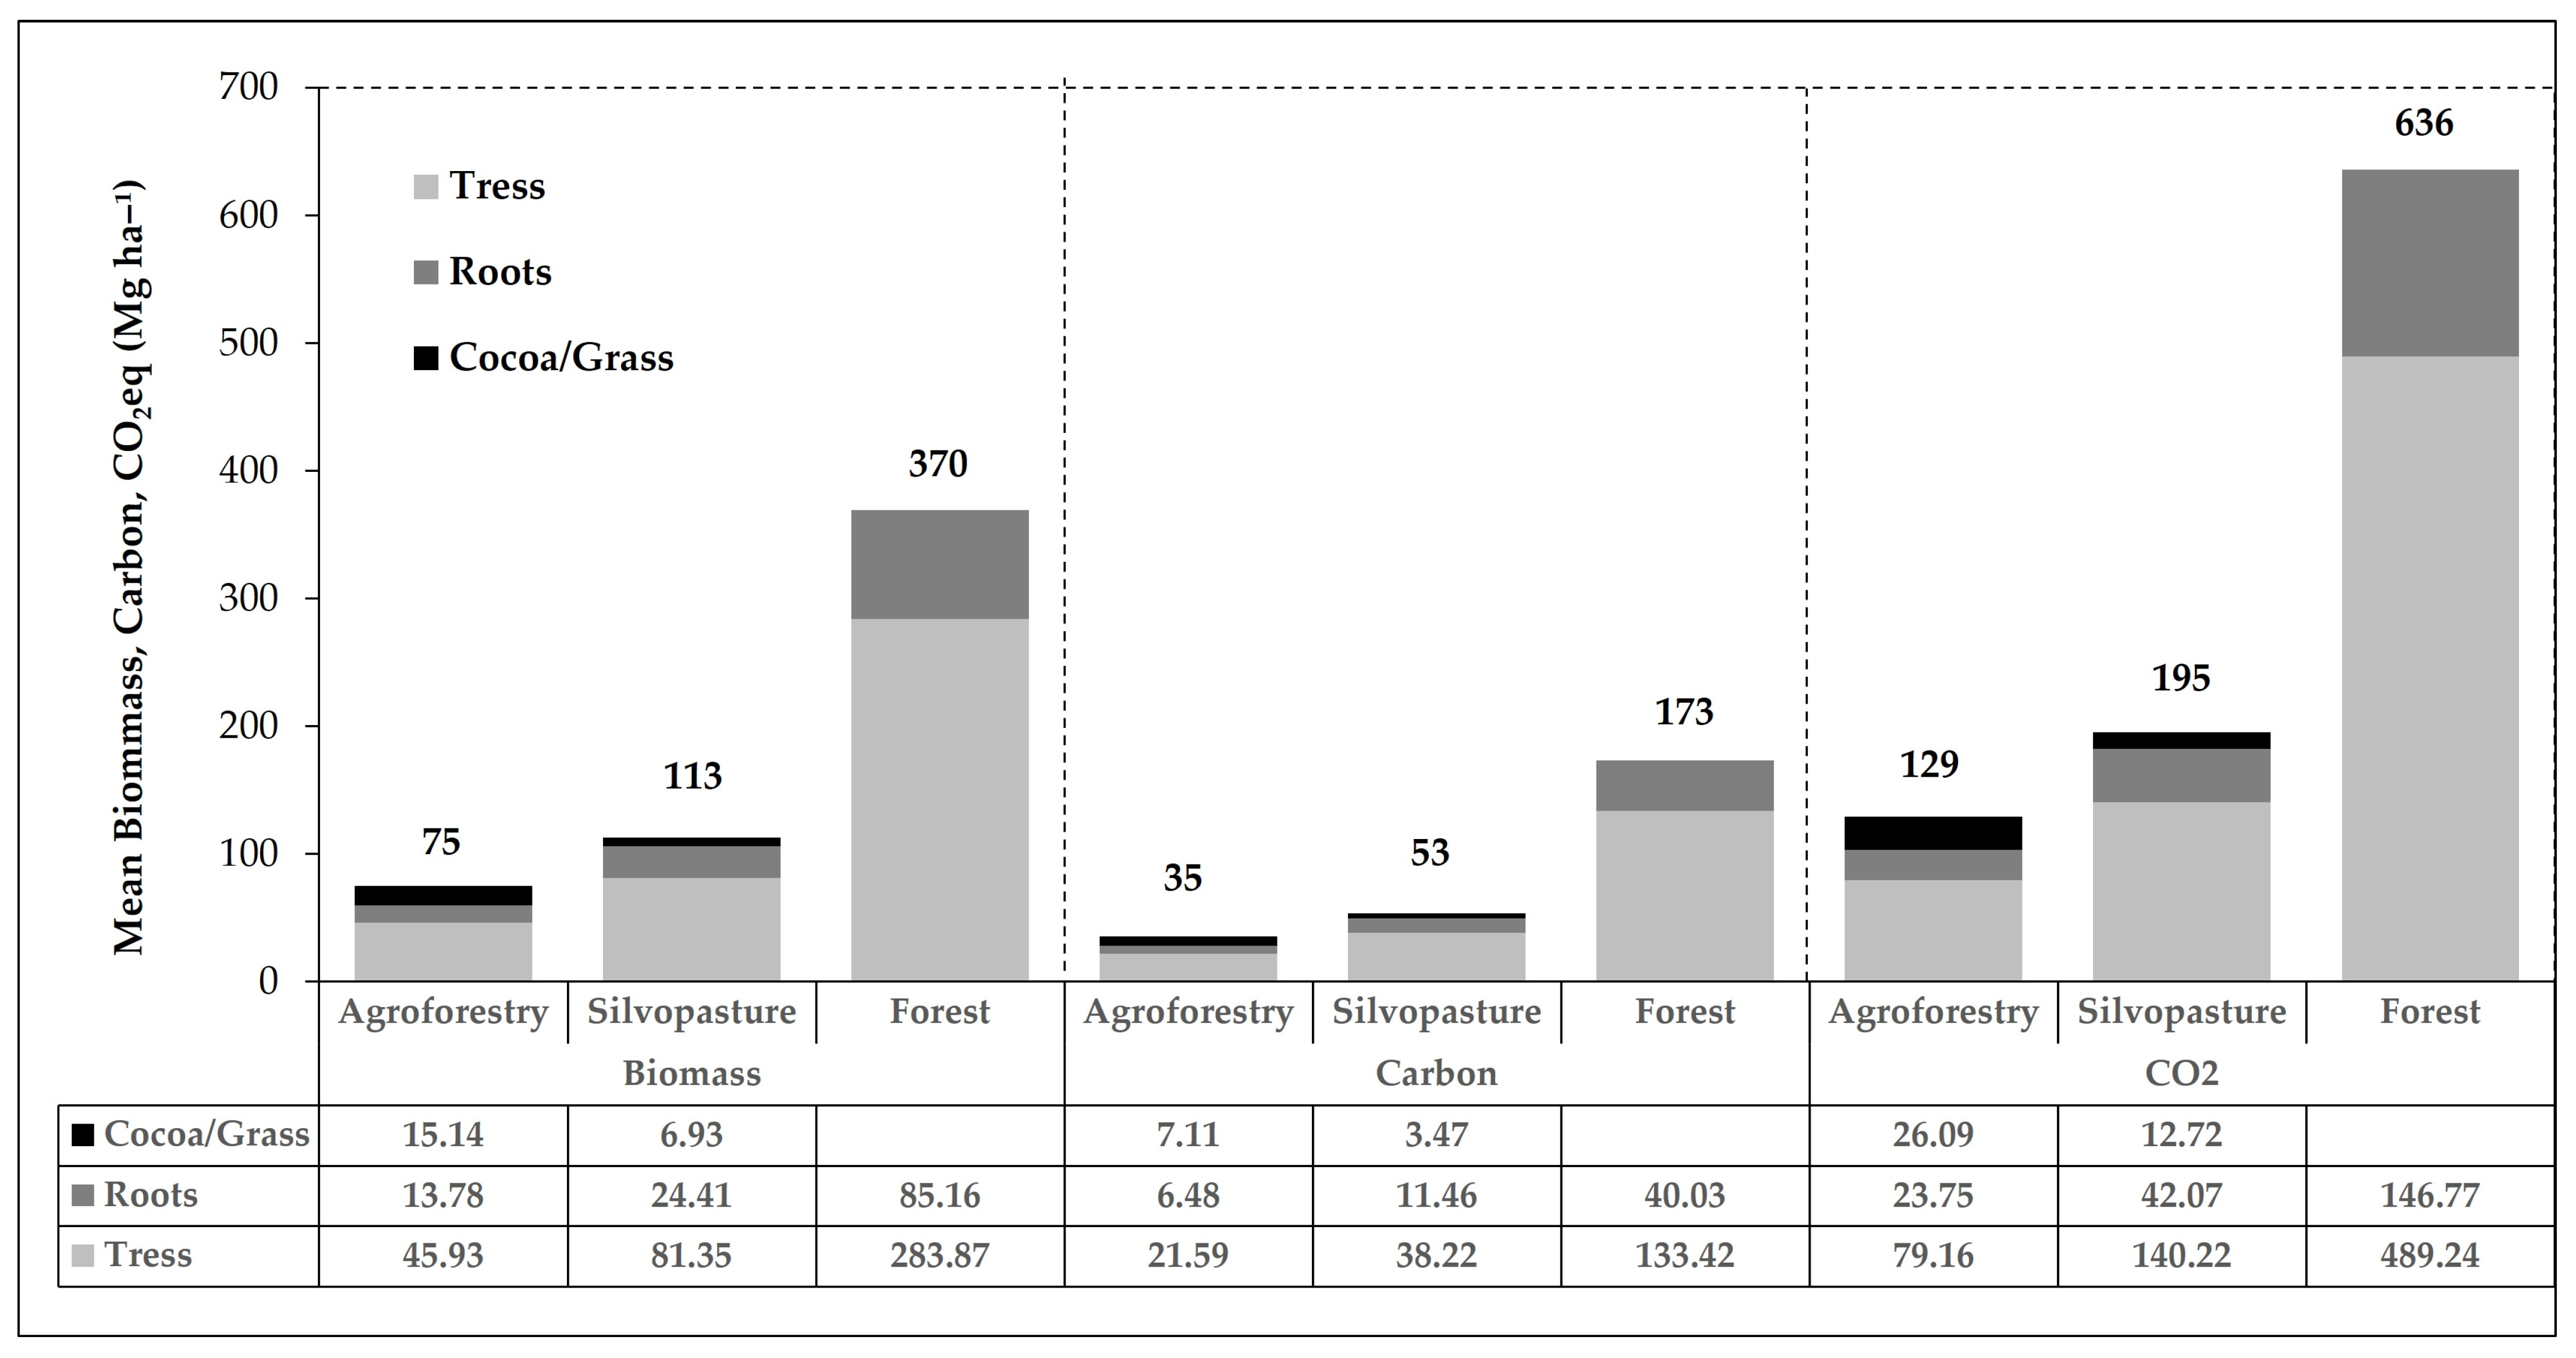
Figure 4 shows clear differences in carbon allocation among land uses. Forests stored the highest carbon stocks, with 133.4 Mg C ha−1 in tree biomass and 40.0 Mg C ha−1 in roots, totaling 173.4 Mg C ha−1 (≈636 Mg CO2 ha−1). In comparison, silvopastoral systems accumulated 37.9 Mg C ha−1 in trees and 11.5 Mg C ha−1 in roots (49.3 Mg C ha−1 total), whereasagroforestry systems stored 21.6 and 6.5 Mg C ha−1 in the same compartments (28.1 Mg C ha−1 total). This distribution reinforces the role of trees as the dominant carbon pool across all land-use systems.
Minor carbon contributions from cacao shrubs in AFS (7.1 Mg C ha−1) and pasture biomass in SPS (3.5 Mg C ha−1) represented less than 10% of total system carbon but confirmed the presence of additional non-tree pools. This pattern suggests that non-tree components play a secondary role in total carbon storage, while tree biomass and roots account for mostretained carbon. Overall, SPS and AFS retained approximately 20–30% (including cacao shrubs and pasture biomass) of forest carbon stocks, mainly through the preservation of remnant trees and their root systems.

4.3. Tree Species Contribution to Carbon and CO2 Stocks

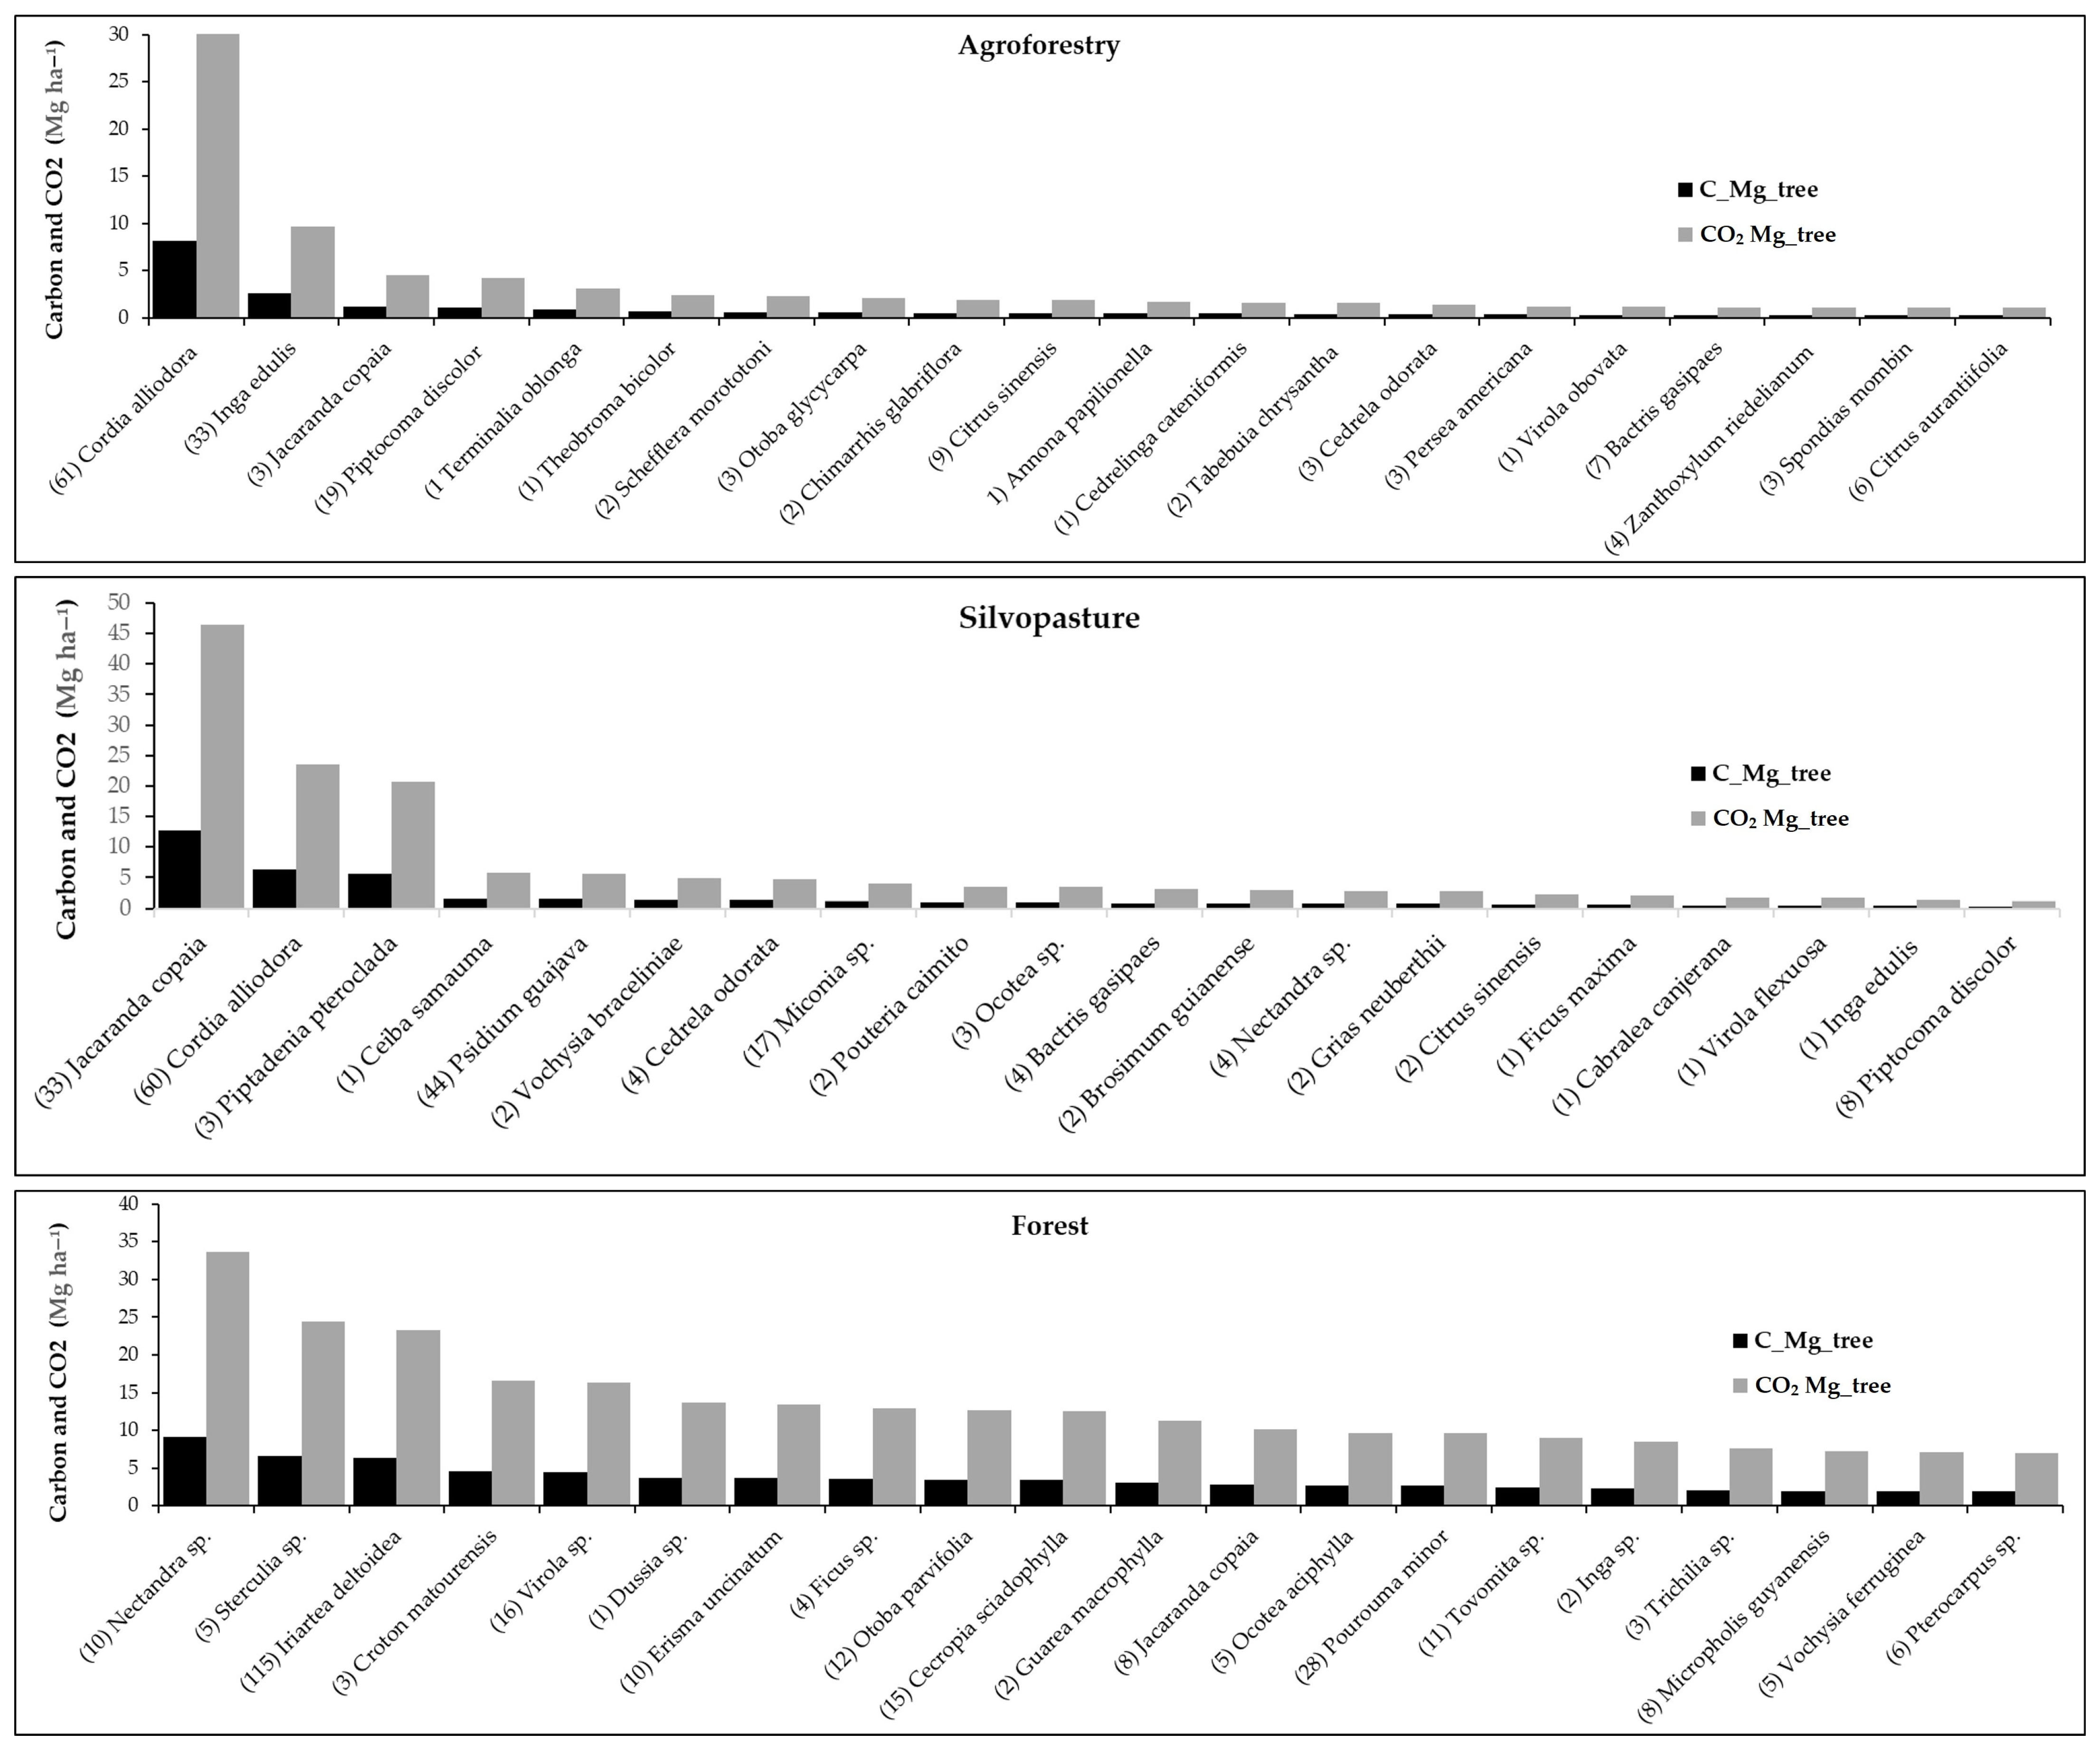
A limited subset of tree species accounted for a disproportionate share of aboveground carbon and CO2-equivalent stocks across all land-use systems (Figure 5). In old-growth forest plots, carbon storage was concentrated in a small group of large-stature, high wood-density taxa—such as Nectandra sp., Sterculia sp., Iriartea deltoidea, and Virola sp.—which dominated biomass accumulation. In agroforestry and silvopastoral systems, total system-level carbon stocks were similarly concentrated within a reduced number of abundant species. Specifically, the nine most abundant species in agroforestry systems and eight species in silvopastoral systems represented approximately 80% of total aboveground CO2-equivalent stocks when aggregated across plots. These taxa also exhibited high basal area and stem density, indicating strong structural influence on biomass distribution within productive land uses.

4.4. Biocultural Patterns of Tree Species Retention and Conservation Status

A total of 151 tree species (DBH ≥ 10 cm) were recorded across the 28 sampling plots, with marked differences in species richness among land-use systems (Table 3). Forest plots exhibited the highest diversity (122 species), followed by Chakra agroforestry systems (35 species) and traditional silvopastoral systems (28 species), reflecting a pronounced richness gradient from forest to productive land uses.
Species abundance patterns differed substantially across land uses (Table 4). While forest plots showed a more even and taxonomically diverse assemblage, agroforestry and silvopastoral systems were dominated by a limited number of species. When ranked by their combined abundance in agroforestry and silvopastoral systems, the Top 20 species accounted for most tree individuals retained in productive land uses, indicating selective retention associated with management practices rather than passive forest remnants.
Across these dominant species, multiple livelihood-related uses were documented, including food provision, medicinal applications, cultural or spiritual functions, and material or timber uses (Table 4). Several of the most abundant taxa in agroforestry and silvopastoral systems—such as Cordia alliodora, Inga edulis, Bactris gasipaes, and Psidium guajava—exhibited more than one documented use category, whereas other dominant species were primarily associated with material or timber functions.
From a conservation and functional attributes perspective, most species actively retained in agroforestry and silvopastoral systems were classified as Least Concern (LC) under IUCN criteria (Table 4). However, a smaller subset of species of higher conservation relevance, including Tabebuia chrysantha (Vulnerable) and Cedrela sp., occurred at low densities across productive systems and forests. Wood density values among retained species spanned a broad range, indicating that agroforestry and silvopastoral systems maintain a functionally diverse but selective subset of tree species present in forest ecosystems.
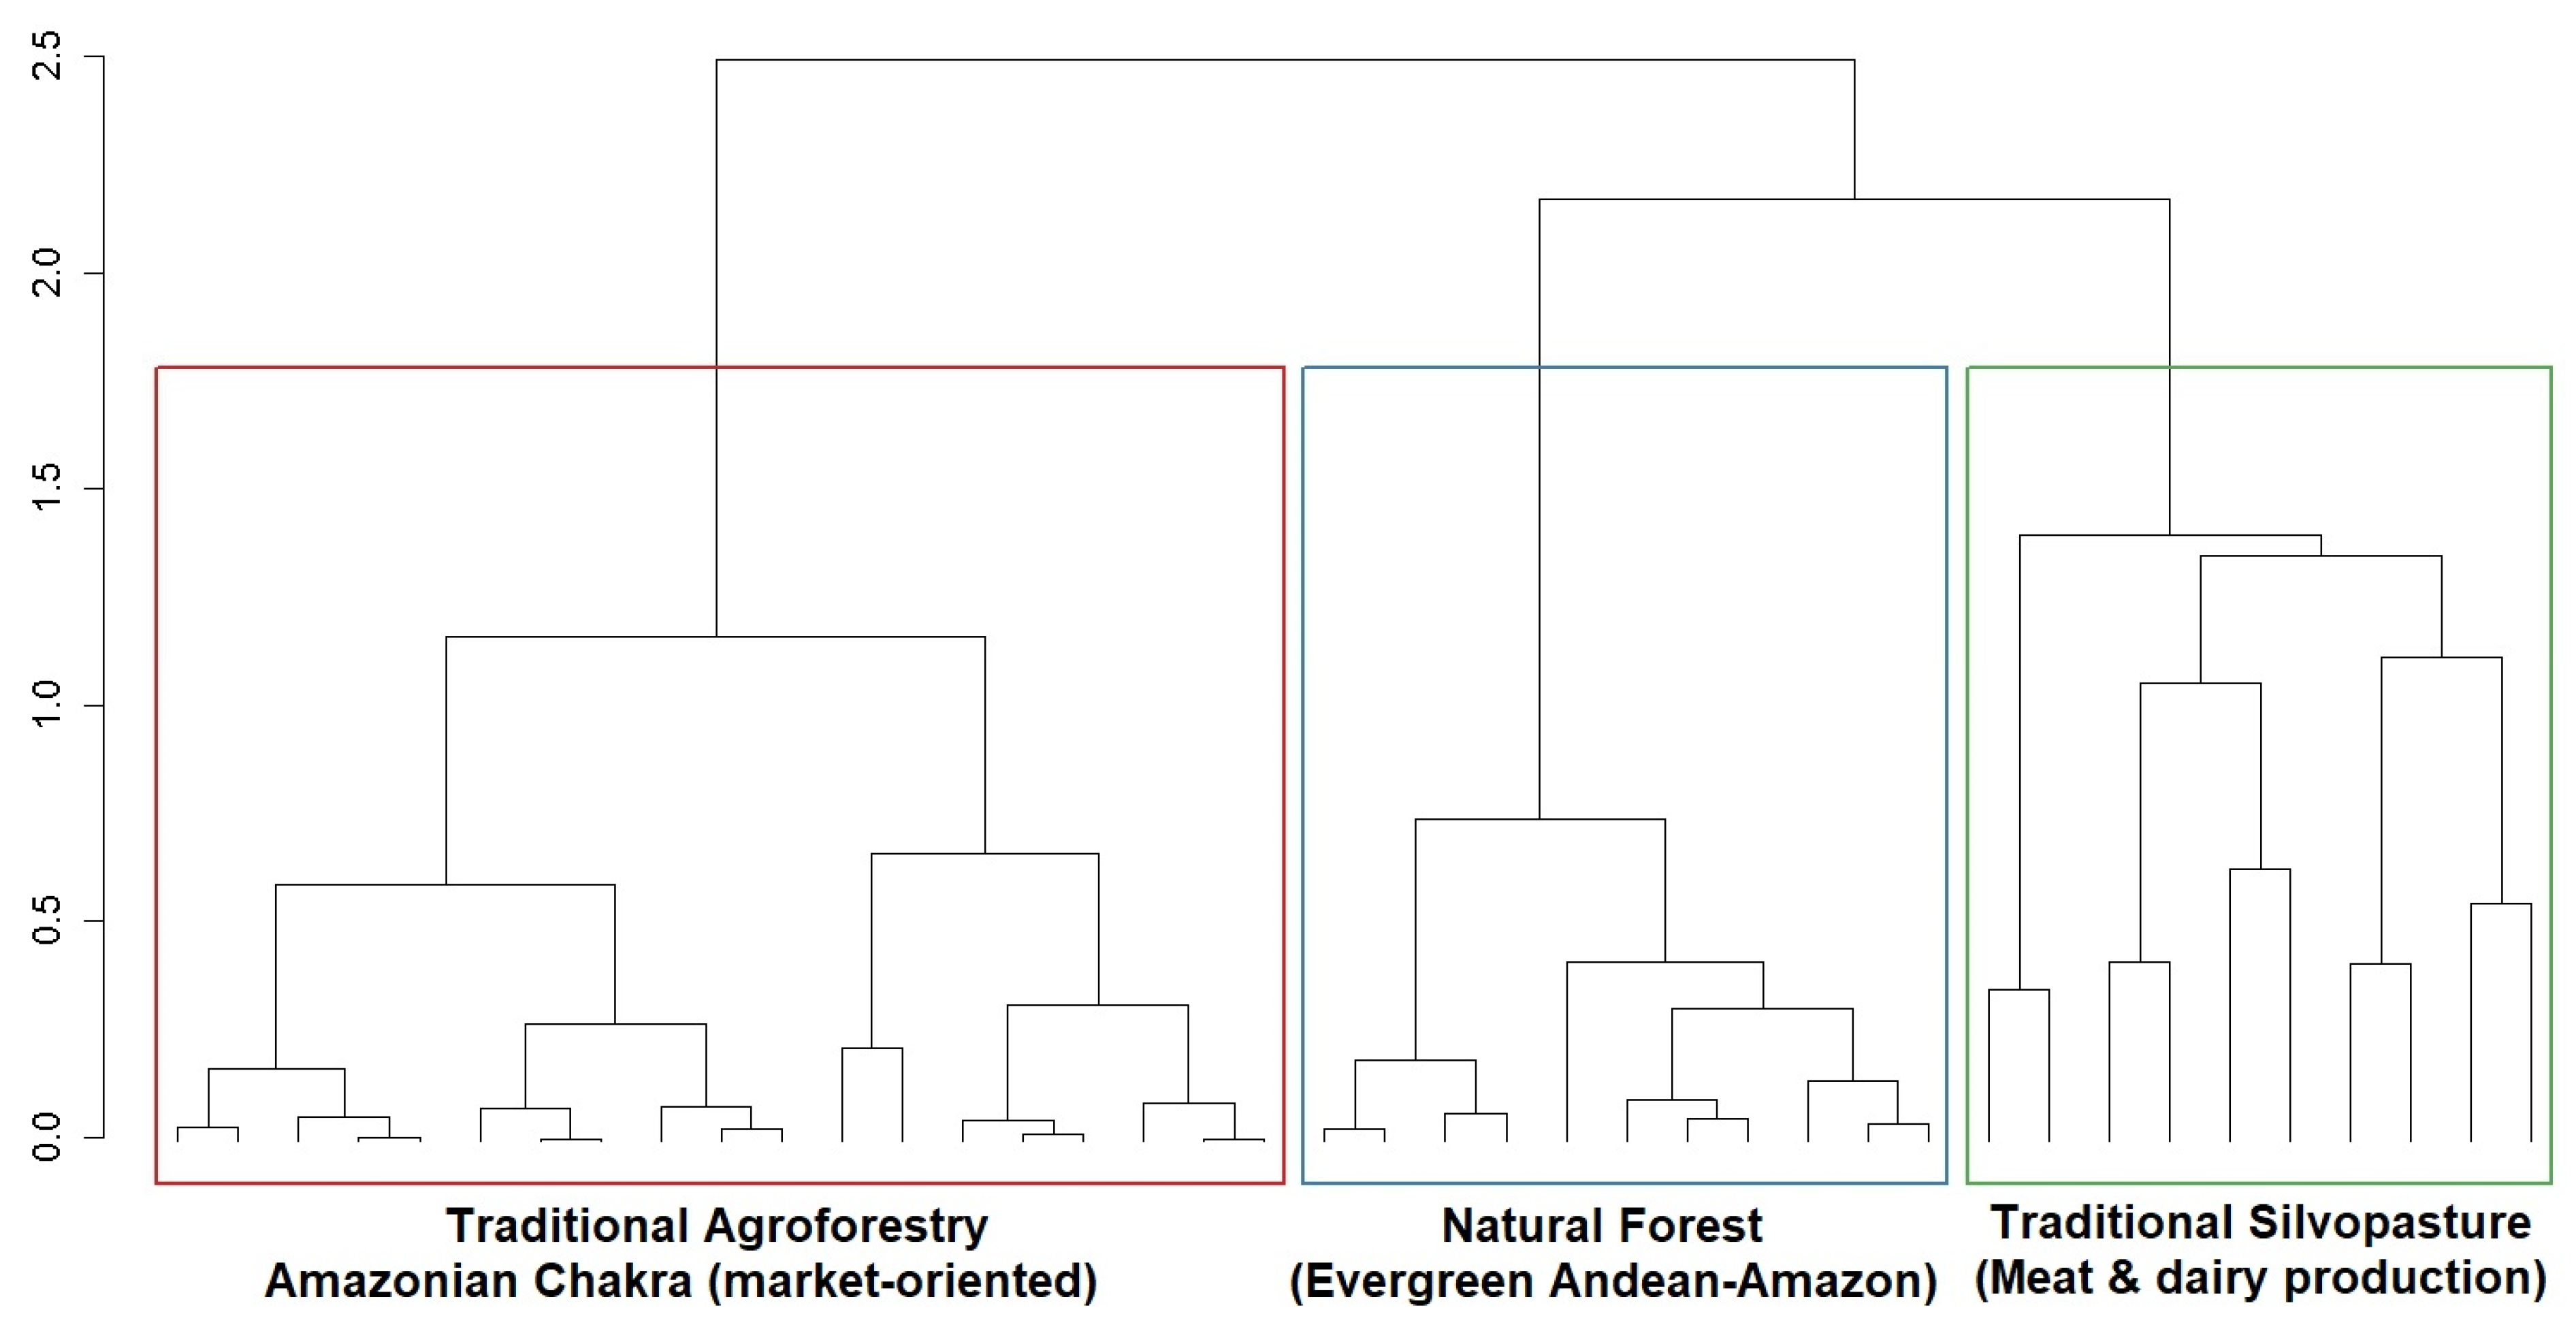
Forest plots contained 122 tree species (DBH ≥ 10 cm), whereas agroforestry and silvopastoral systems retained 35 and 28 species, respectively. Despite this reduction in richness, productive systems did not represent random subsets of forest assemblages. A limited number of dominant taxa accounted for most individuals in managed systems, and hierarchical clustering showed compositional differentiation among land uses. Such dominance patterns are consistent with selective species retention shaped by management practices, a process widely referenced in tropical agroecosystems [13].

5. Discussion

5.1. Carbon Retention in Biocultural Productive Landscapes: Forests, Agroforestry, and Silvopasture

The results indicate that traditional Chakra AFS and traditional SPS, embedded within an evergreen Andean–Amazon forest landscape in Arosemena Tola, retain substantial amounts of carbon, supporting their relevance as climate-smart, tree-based production systems [36]. As expected, old-growth forests stored the highest aboveground carbon stocks, with values approximately three to six times higher than those recorded in AFS and SPS [29,30]. Nevertheless, productive systems maintained meaningful carbon reserves, far exceeding those reported for monocultures or treeless pastures [1]. These findings directly address Objective 1, showing that AFS and SPS retain approximately 20–30% of forest carbon stocks, thereby preserving a non-trivial structural legacy within managed landscapes [49].
Beyond proportional carbon retention (20–30%), these patterns reflect structured outcomes of selective tree retention rather than passive ecological persistence. In both agroforestry and silvopastoral systems, large-diameter and multifunctional species are disproportionately maintained, concentrating biomass within a reduced subset of dominant taxa. Although individuals exceeding 40 cm DBH represent a relatively small fraction of total stems in managed systems, they account for a substantial share of total carbon stocks, indicating a pronounced size-class concentration effect. Such configurations are consistent with documented management strategies in tropical tree-based systems, where producers balance shade provision, timber value, system stability, and productive performance through intentional species selection [12,13,27,40]. Under these conditions, carbon accumulation emerges not solely from successional processes but from culturally embedded, livelihood-oriented decision-making that shapes structural composition over time.
The relatively minor contribution of cocoa shrubs and pasture grasses (<10% of total carbon stock) further underscores the structural dominance of the arboreal component in these systems. Carbon retention in both agroforestry and silvopastoral landscapes is therefore primarily driven by tree presence, size distribution, and biomass concentration rather than by understory or pasture biomass. This finding reinforces the importance of maintaining arboreal structural complexity within productive land uses.
Species-level patterns help explain the mechanisms underpinning carbon retention. As illustrated in Figure 5, carbon stocks across all land-use systems were disproportionately concentrated in a limited number of dominant tree species, highlighting the strong influence of structural attributes on biomass accumulation [49,63]. In forest plots, this pattern was driven by large-stature species with high wood density, whereas in AFS and SPS, it reflected the selective retention of multifunctional taxa, such as Cordia alliodora, Inga edulis, Jacaranda copaia, and Piptocoma discolor, consistent with patterns reported for Amazonian agroforestry systems [11,12,15]. In the regional context of Arosemena Tola, this selective retention reflects long-standing management practices adapted to humid Andean–Amazon conditions rather than opportunistic tree persistence. Consistent with this pattern, Table 3 shows that the most abundant species retained in productive systems combine material, food, medicinal, and cultural uses with intermediate to high wood density values, reinforcing their dual ecological and livelihood functions [64].
Notably, the Amazonian Chakra system analyzed here corresponds to a traditional cacao-based agroforestry system oriented to market production, while maintaining associated tree species linked to food security and cultural uses. This configuration, observed under the specific biophysical and socio-cultural conditions of the Andean–Amazon transition zone, supports previous evidence that economically viable traditional agroforestry systems can reduce pressures toward land-use simplification and monoculture expansion, thereby contributing to the persistence of biocultural management practices in Indigenous landscapes [10,35].
At the landscape scale, these patterns indicate that AFS and SPS contribute to the structural continuity of carbon stocks beyond forest boundaries, supporting a continuous, albeit heterogeneous, carbon network along the forest–agriculture gradient [27,36]. Within the regional scope of this study, this finding supports Objective 3, underscoring the importance of recognizing tree-based production systems as complementary components of Nature-Based Solutions that integrate carbon retention, biodiversity, and local livelihoods within biocultural productive landscapes.

5.2. Functional Diversity and Biocultural Species Selection in Tree-Based Productive Systems

AFS and SPS in the Andean–Amazon landscape maintains distinctive combinations of tree diversity and functional traits as a result of intentional species selection, rather than passive ecological persistence. As shown in Table 3, many dominant species retained in productive systems combine multiple livelihood-related uses (food, medicinal, cultural, and material) with functional traits relevant to system performance, including intermediate to high wood density and rapid growth. This pattern indicates that species composition in AFS and SPS is shaped by biocultural decision-making, in which ecological functionality and livelihood benefits are jointly optimized, as documented for other Amazonian tree-based systems [10,11,12]. These results directly support Objective 1 and Objective 2 by demonstrating that structural attributes and floristic composition influence carbon storage and that these patterns are shaped by local management decisions rather than stochastic processes.
In agroforestry systems, multifunctional species such as Cordia alliodora, Inga edulis, Jacaranda copaia, and Piptocoma discolor dominate tree assemblages and contribute disproportionately to structural complexity. These species provide shade, timber, soil fertility enhancement, and other ecosystem functions [13,46,49], while sustaining household production goals, exemplifying a process of functional species filtering widely reported in Amazonian biocultural landscapes [14,15]. Similarly, silvopastoral systems retain tree assemblages characterized by structurally and functionally valuable species, reflecting intentional ecological design aimed at balancing forage production with shade provision [26,32], timber value [31], and long-term system stability, rather than opportunistic tree persistence [47,58].
Multivariate patterns of species composition further reinforce this interpretation. The hierarchical clustering analysis (Figure 6) shows that forest, agroforestry, and silvopastoral plots form floristically distinct yet internally coherent clusters rather than following a simple linear degradation gradient. While forest plots cluster due to higher richness and evenness, AFS and SPS each form assemblages structured primarily by management practices. This supports the characterization of tree-based productive systems as working forests, which retain key ecological attributes of natural forests—such as structural heterogeneity and functional diversity—even when embedded within agricultural matrices [30,36,65].
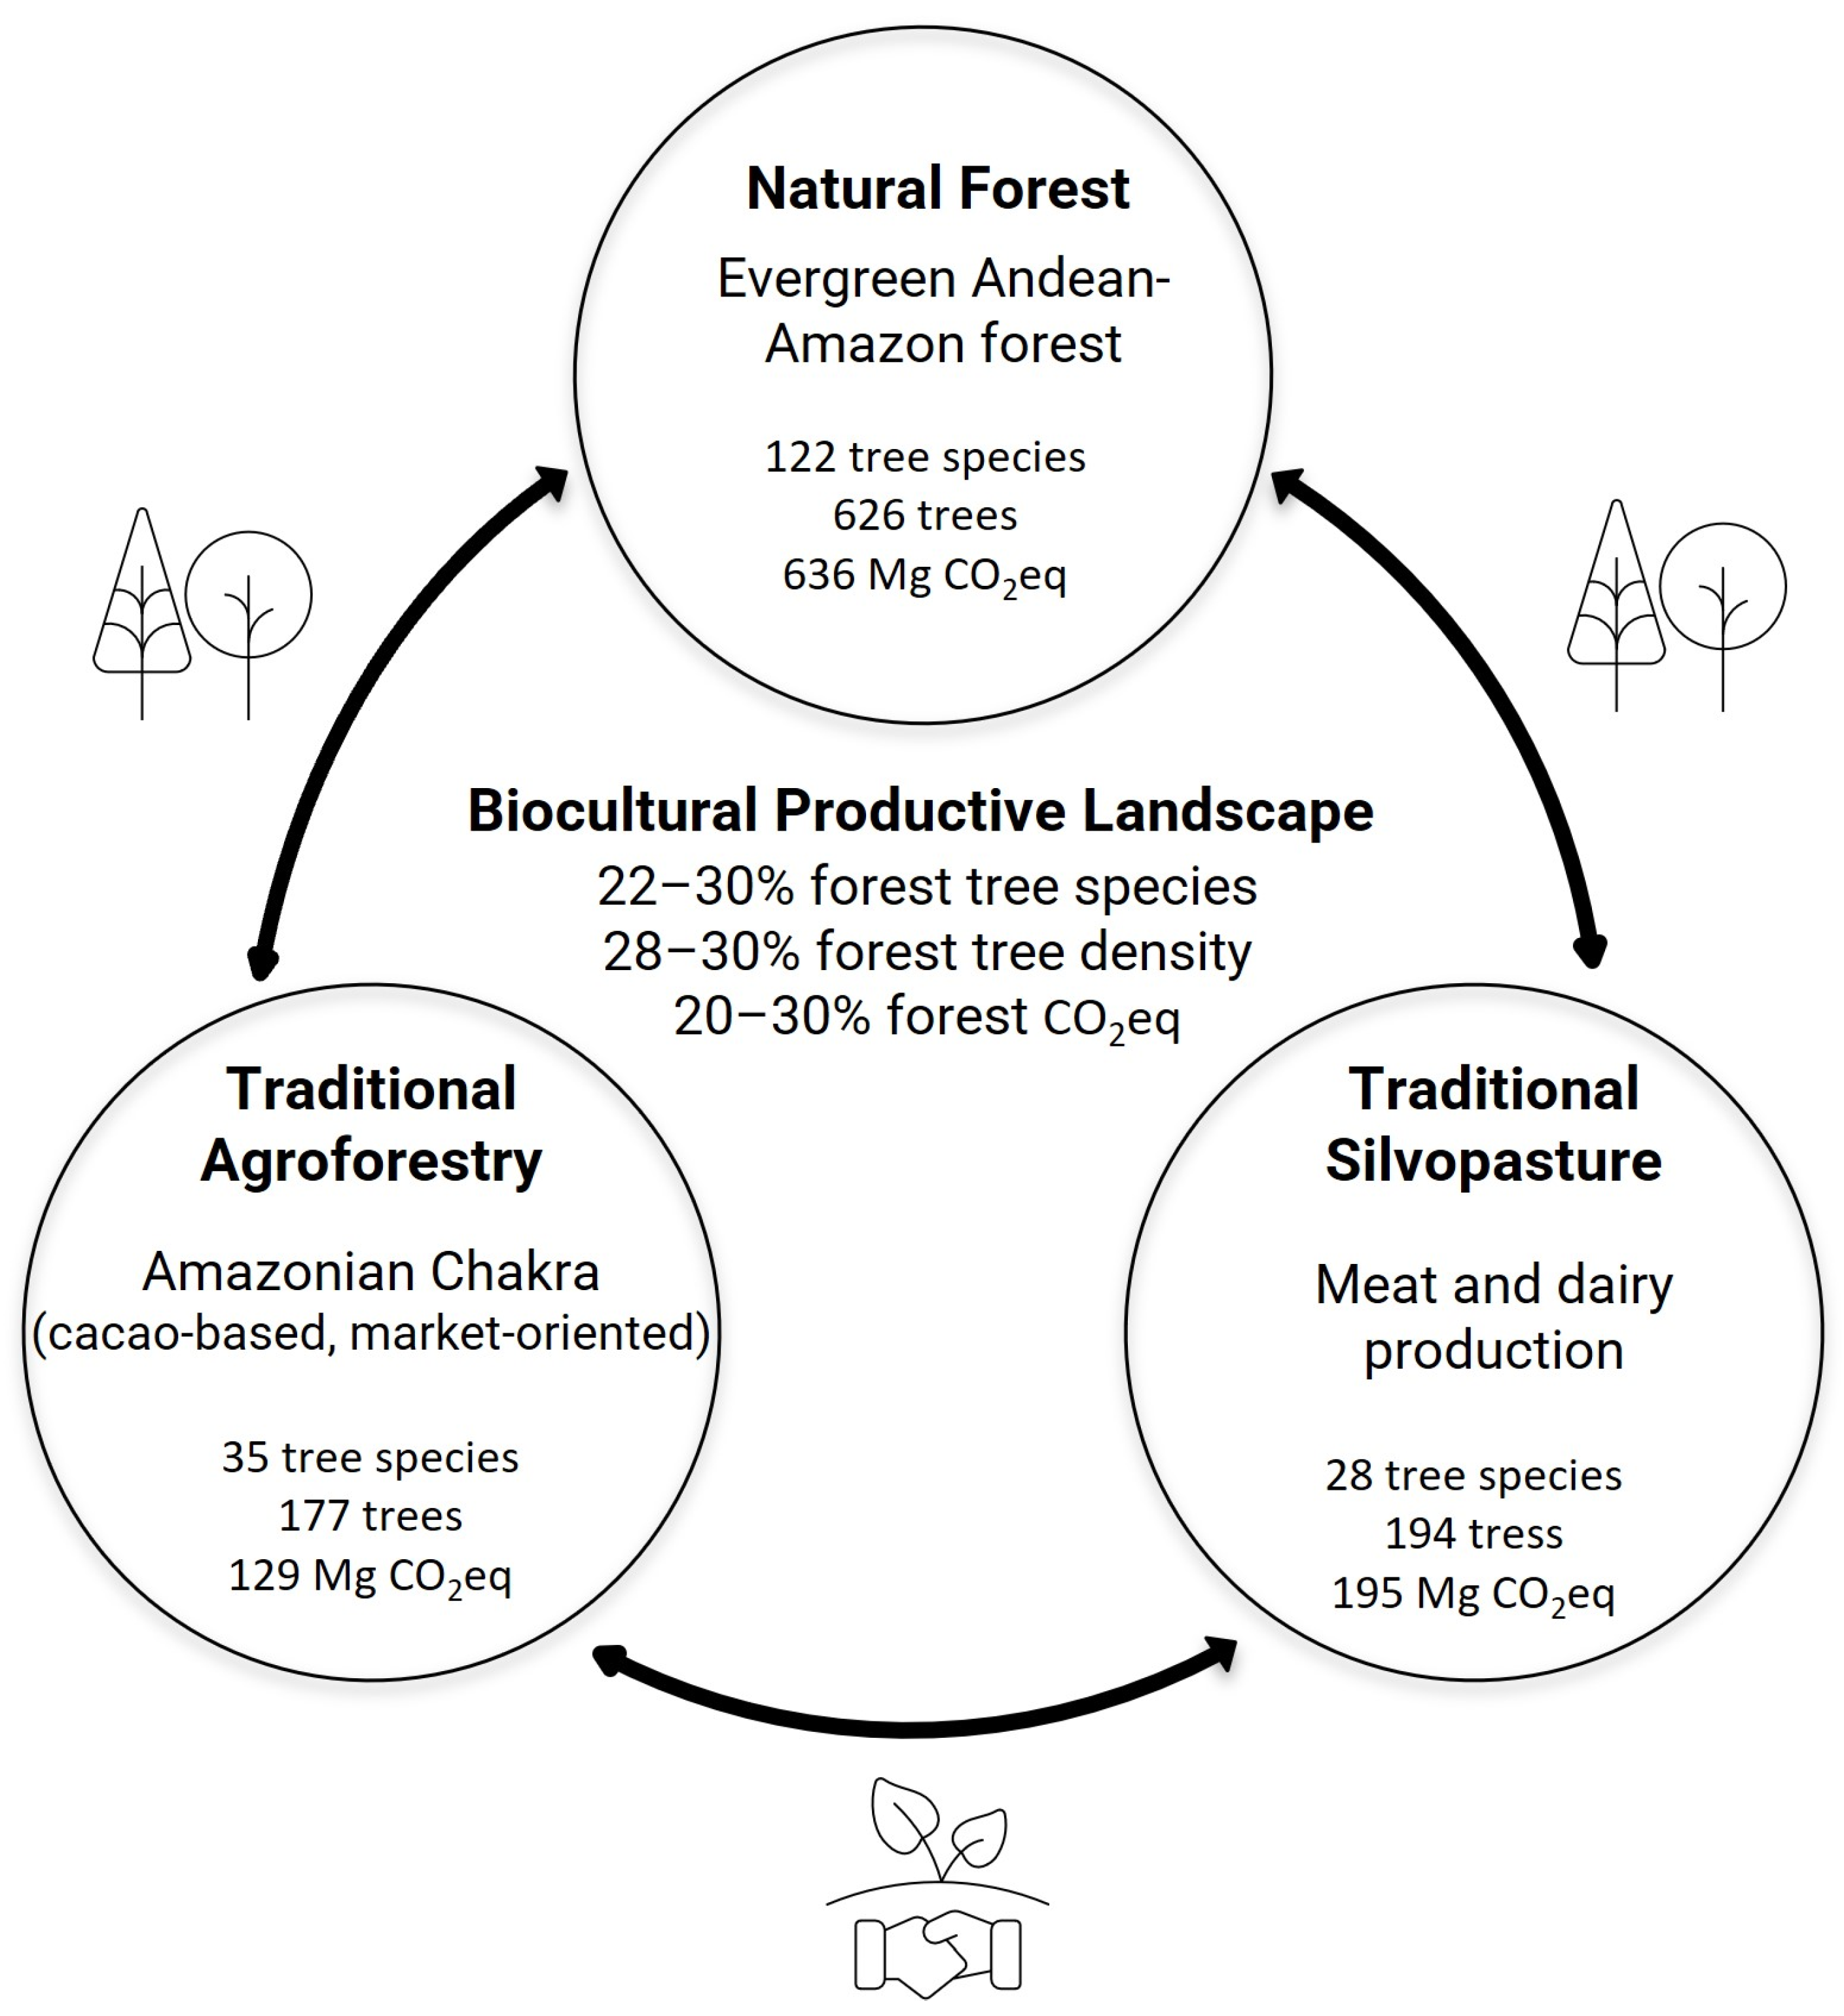
The relationships among forest, agroforestry, and silvopastoral systems are further synthesized in the conceptual model presented in Figure 7, which frames these land uses as interconnected components of a biocultural productive landscape rather than as stages along a unidirectional deforestation pathway. Although natural forests retain the highest levels of tree species richness and aboveground carbon stocks, both agroforestry and silvopastoral systems conserve substantial proportions of forest attributes, including approximately 22–30% of tree species richness, 28–30% of tree density, and 20–30% of forest aboveground carbon. Notably, the species retained are not random subsets but multifunctional taxa that contribute to structural carbon and livelihood functions, reflecting selective retention shaped by management priorities rather than incidental simplification [27,36].
Differences in plot configuration and area among land-use systems, the use of generalized allometric models and standard coefficients for BGB, and the absence of explicit spatial connectivity metrics may introduce uncertainty in absolute biomass and carbon estimates. Furthermore, this research was intentionally designed as a site-scale comparative assessment within a specific Andean–Amazon mosaic and therefore does not capture the full ecological, cultural, or management variability present across broader Amazonian regions.
Although these methodological considerations may affect absolute stock magnitudes, the consistent sampling framework, per-hectare standardization, and replicated design across land-use types support the robustness of the relative structural, compositional, and carbon-retention patterns observed within the study landscape. Accordingly, interpretations are restricted to within-mosaic comparisons among the evaluated systems and should not be extrapolated to larger spatial or regional scales without additional empirical validation.
Future research should extend this analytical framework to multiple sites and broader spatial scales, incorporate landscape-level connectivity metrics, and develop system-specific belowground biomass estimates. Such efforts would allow testing the generality of the BPL framework under varying ecological and socio-cultural contexts, thereby strengthening its applicability beyond this case study.

5.3. Toward Policy Recognition and Incentives for Tree-Based Production Landscapes

Despite the recent international recognition of the Amazonian Chakra through its designation as a Globally Important Agricultural Heritage System (GIAHS), traditional silvopastoral systems embedded within the same Andean–Amazonian cultural landscapes remain largely overlooked by conservation and climate policy frameworks. Within the Andean–Amazon regional context examined in this study, this asymmetry persists even though SPS exhibits comparable levels of tree cover, ecological functionality, and carbon retention to agroforestry systems, as indicated by the empirical evidence presented here. Such imbalance may reflect broader policy dynamics across the Amazon, where forest conservation has traditionally been prioritized, while tree-based production systems are rarely acknowledged as legitimate contributors to climate mitigation, biodiversity conservation, or landscape restoration [21,36]. This forest-centric bias aligns with critiques articulated in Nature’s Matrix, which emphasize how tropical conservation policies have historically favored “fortress forest” approaches centered on strict forest protection and the exclusion of productive tree-based landscapes at the expense of multifunctional, tree-rich agricultural systems [13]. In contrast, both agroforestry and silvopastoral systems documented in this study can be interpreted as examples of what recent Amazon governance debates describe as vernacular climate solutions, namely locally rooted land-use systems that integrate carbon retention, biodiversity conservation, food production, and socio-cultural continuity [28]. Rather than being considered degraded or merely transitional land uses within this regional setting, these systems reflect long-standing biocultural management strategies that actively sustain ecosystem functions within working landscapes.
At the policy level, these findings may be relevant for informing ongoing regional and global agendas, including the Belém Declaration (2023) and contemporary socio-bioeconomy proposals for the Amazon, which emphasize scaling up existing biocultural practices rather than replacing them with externally imposed land-use models [28,66]. However, within the current policy landscape, access to financial and institutional support remains uneven. While agroforestry systems have increasingly benefited from payment for ecosystem services (PES) schemes, differentiated certifications, and, in some cases, voluntary carbon markets, silvopastoral systems—despite retaining approximately 30% of forest carbon stocks (expressed as CO2-equivalent per hectare) and supporting native tree diversity—remain largely excluded from GIAHS pathways, REDD+ eligibility criteria, and most climate finance instruments [23].
Addressing this policy gap could involve consideration of a strategic shift away from forest-status–based incentives toward tree-cover– and functionality–based incentive frameworks capable of recognizing carbon storage, biodiversity conservation, and restoration outcomes across heterogeneous land uses. Such approaches include carbon credit mechanisms accessible to smallholders, biodiversity payments linked to tree retention, and tailored financing instruments for livestock systems that maintain or restore arboreal structure, as proposed by Montagnini et al. [67] and Torres et al. [68]. Comparable models are already being piloted in other tropical regions, where eligibility for ecosystem service payments is determined by measurable tree presence and functional attributes rather than by binary land-use classifications.
Based on the empirical results obtained, both agroforestry and silvopastoral systems merit formal consideration within nationally determined contributions (NDCs), climate-smart agriculture strategies, and biocultural heritage policies. Far from being secondary or residual land uses, these systems can be viewed as tree-based livelihood systems with high climate value, cultural legitimacy, and restoration potential at the regional scale. In this context, traditional silvopastoral systems of the Andean–Amazon region emerges as potential candidates for future GIAHS recognition, not as substitutes for natural forests but as co-producing landscapes that complement forest conservation while sustaining carbon retention, biodiversity, and local knowledge.

6. Conclusions

This study demonstrates that traditional tree-based production systems in the Andean–Amazon transition zone retain approximately 20–30% of the aboveground carbon stocks of old-growth forests while maintaining key ecological functions and biocultural management practices. Although structurally less complex than primary forests, these systems sustain diverse assemblages of multipurpose tree species that contribute to carbon storage, habitat continuity, and livelihood resilience across managed landscapes.
Specifically, the findings show that (i) tree diversity, structural attributes, and carbon stocks differ significantly among forest, agroforestry, and silvopastoral systems; (ii) carbon storage in productive systems is largely driven by a limited number of multifunctional tree species intentionally retained through biocultural management, resulting in a pronounced concentration of biomass in structurally dominant individuals; and (iii) both agroforestry and silvopastoral systems contribute to structural continuity within forest–agriculture mosaics by maintaining tree cover and associated ecological functions. Their configuration indicates potential contributions to landscape connectivity, warranting further research on functional and spatial dynamics across broader scales.
Overall, the results provide case-based empirical support for the BPL framework within the Andean–Amazon context examined here. Carbon retention in productive systems is not randomly distributed but reflects culturally mediated species selection that balances livelihood functions with ecological performance. In this sense, agroforestry and silvopastoral systems operate as integrated components of biocultural landscapes, sustaining measurable carbon stocks and biodiversity beyond forest boundaries.
From a broader perspective, these findings suggest that sustainable Amazonian futures will depend not only on protecting remaining forests but also on strengthening multifunctional, culturally informed production systems embedded in surrounding landscapes. While the Amazonian Chakra has received international recognition as a Globally Important Agricultural Heritage System (GIAHS), traditional silvopastoral systems remain largely absent from conservation and climate finance frameworks despite evidence of comparable ecological and carbon value. Integrating tree-based productive systems into national and subnational climate strategies, carbon accounting approaches, and incentive mechanisms—such as REDD+, payments for ecosystem services, and agroecological certification—could foster more inclusive and territorially grounded pathways toward Amazonian sustainability.

Author Contributions

Conceptualization, B.T.; methodology, B.T., A.G. and A.T.; software, B.T.; validation, R.H.-F., J.M.-R. and C.T.-T.; formal analysis, B.T.; investigation, B.T., J.M.-R., C.T.-T., R.H.-F. and A.T.; data curation B.T. and H.R.; writing—original draft preparation, B.T., J.M.-R., C.T.-T., R.H.-F. and A.T.; writing—review and editing, B.T.; A.G., H.R., A.T., C.T.-T. and J.M.-R.; supervision B.T. and A.G. All authors have been involved in developing, writing, commenting, editing, and reviewing the manuscript. All authors have read and agreed to the published version of the manuscript.

Funding

This research received no external funding.

Institutional Review Board Statement

Not applicable.

Informed Consent Statement

Not applicable.

Data Availability Statement

The original contributions presented in this study are included in the article. Further inquiries can be directed to the corresponding authors.

Acknowledgments

The authors thank the MAG, MAE, UEA, UTEQ for their support during the fieldwork stage, as well as the households in the three land-use systems that shared valuable information.

Conflicts of Interest

Authors Bolier Torres and Cristhian Tipán-Torres are affiliated with Ochroma Consulting & Services in addition to their academic institutions. The remaining authors declare that the research was conducted in the absence of any commercial or financial relationships that could be construed as a potential conflict of interest.

References

  1. Gibbs, H.K.; Ruesch, A.S.; Achard, F.; Clayton, M.K.; Holmgren, P.; Ramankutty, N.; Foley, J.A. Tropical Forests Were the Primary Sources of New Agricultural Land in the 1980s and 1990s. Proc. Natl. Acad. Sci. USA 2010, 107, 16732–16737. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  2. Bartolini, F.; Andreoli, M.; Brunori, G. Explaining Determinants of the On-Farm Diversification: Empirical Evidence from Tuscany Region. Bio-Based Appl. Econ. 2014, 3, 137–157. [Google Scholar] [CrossRef] [Scilit]
  3. Tilman, D.; Balzer, C.; Hill, J.; Befort, B.L. Global Food Demand and the Sustainable Intensification of Agriculture. Proc. Natl. Acad. Sci. USA 2011, 108, 20260–20264. [Google Scholar] [CrossRef] [Scilit]
  4. Seufert, V.; Ramankutty, N.; Foley, J.A. Comparing the Yields of Organic and Conventional Agriculture. Nature 2012, 485, 229–232. [Google Scholar] [CrossRef] [Scilit]
  5. Montagnini, F.; Metzel, R. The Contribution of Agroforestry to Sustainable Development Goal 2: End Hunger, Achieve Food Security and Improved Agricultura Nutrition, and Promote Sustainable Agriculture; Springer International Publishing: Berlin/Heidelberg, Germany, 2017; ISBN 9783319693712. [Google Scholar]
  6. De Macêdo Carvalho, C.B.; de Mello, A.C.L.; da Cunha, M.V.; de Oliveira Apolinário, V.X.; Dubeux, J.C.B.; da Silva, V.J.; Medeiros, A.S.; Izidro, J.L.P.S.; Bretas, I.L. Ecosystem Services Provided by Silvopastoral Systems: A Review. J. Agric. Sci. 2024, 162, 417–432. [Google Scholar] [CrossRef] [Scilit]
  7. Montagnini, F.; del Fierro, S. Functions of Agroforestry Systems as Biodiversity Islands in Productive Landscapes. In Biodiversity Islands: Strategies for Conservation in Human-Dominated Environments; Springer: Berlin/Heidelberg, Germany, 2022; pp. 89–116. [Google Scholar]
  8. Vera-Vélez, R.; Grijalva, J.; Cota-Sánchez, J.H. Cocoa Agroforestry and Tree Diversity in Relation to Past Land Use in the Northern Ecuadorian Amazon. New For. 2019, 50, 891–910. [Google Scholar] [CrossRef] [Scilit]
  9. Díaz-Cháux, J.T.; Velasquez-Valencia, A.; Casanoves, F. Influence of Landscape Structure on Carbon Storage in Agroforestry Systems with Cacao and Silvopastoral Systems in the Colombian Amazon. PLoS ONE 2025, 20, e0325477. [Google Scholar] [CrossRef] [Scilit]
  10. Kremen, C.; Merenlender, A.M. Landscapes That Work for Biodiversity and People. Science 2018, 362, eaau6020. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  11. Hong, S.K. Biocultural Diversity Conservation for Island and Islanders: Necessity, Goal and Activity. J. Mar. Isl. Cult. 2013, 2, 102–106. [Google Scholar] [CrossRef] [Scilit]
  12. Altieri, M.A. Linking Ecologists and Traditional Farmers in the Search for Sustainable Agriculture. Front. Ecol. Environ. 2004, 2, 35–42. [Google Scholar] [CrossRef]
  13. Perfecto, I.; Vandermeer, J. The Agroecological Matrix as Alternative to the Land-Sparing/Agriculture Intensification Model. Proc. Natl. Acad. Sci. USA 2010, 107, 5786–5791. [Google Scholar] [CrossRef] [Scilit]
  14. Coq-Huelva, D.; Torres-Navarrete, B.; Bueno-Suárez, C. Indigenous Worldviews and Western Conventions: Sumak Kawsay and Cocoa Production in Ecuadorian Amazonia. Agric. Hum. Values 2018, 35, 163–179. [Google Scholar] [CrossRef] [Scilit]
  15. Coq-Huelva, D.; Higuchi, A.; Alfalla-Luque, R.; Burgos-Morán, R.; Arias-Gutiérrez, R. Co-Evolution and Bio-Social Construction: The Kichwa Agroforestry Systems (Chakras) in the Ecuadorian Amazonia. Sustainability 2017, 9, 1920. [Google Scholar] [CrossRef] [Scilit]
  16. Mittermeier, R.A.; Myers, N.; Thomsen, J.B.; da Fonseca, G.A.B.; Olivieri, S. Biodiversity Hotspots and Major Tropical Wilderness Areas: Approaches to Setting Conservation Priorities. Conserv. Biol. 1998, 12, 516–520. [Google Scholar] [CrossRef] [Scilit]
  17. Mittermeier, R.A.; Myers, N.; Mittermeier, C.G.; Robles Gil, P. Hotspots: Earth’s Biologically Richest and Most Endangered Terrestrial Ecoregions; Cemex: Houston, TX, USA, 1999; ISBN 9686397582. [Google Scholar]
  18. Myers, N.; Mittermeier, R.A.; Fonseca, G.A.B.; Fonseca, G.A.B.; Kent, J. Biodiversity Hotspots for Conservation Priorities. Nature 2000, 403, 853–858. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  19. Ministerio del Ambiente del Ecuador (MAE). Plan de Manejo Del Parque Nacional Sumaco—Napo Galeras; MAE: Quito, Ecuador, 2013; 81p.
  20. Torres, B.; Luna, M.; Tipán-Torres, C.; Ramírez, P.; Muñoz, J.C.; García, A. A Simplified Integrative Approach to Assessing Productive Sustainability and Livelihoods in the “Amazonian Chakra” in Ecuador. Land 2024, 13, 2247. [Google Scholar] [CrossRef] [Scilit]
  21. FAO. Amazonian Chakra—Sistemas Importantes del Patrimonio Agrícola Mundial (SIPAM). Available online: https://www.fao.org/giahs/around-the-world/detail/ecuador-amazonia/en (accessed on 15 October 2025).
  22. Nair, P.K.R.; Kumar, B.M.; Nair, V.D. Silvopastoral Systems (SPS) in the Tropics and Subtropics. In An Introduction to Agroforestry; Springer: Berlin/Heidelberg, Germany, 2021; pp. 169–193. [Google Scholar] [CrossRef] [Scilit]
  23. Bennett, N.J.; Roth, R.; Klain, S.C.; Chan, K.; Christie, P.; Clark, D.A.; Cullman, G.; Curran, D.; Durbin, T.J.; Epstein, G.; et al. Conservation Social Science: Understanding and Integrating Human Dimensions to Improve Conservation. Biol. Conserv. 2017, 205, 93–108. [Google Scholar] [CrossRef] [Scilit]
  24. República del Ecuador. Segunda Contribución Determinada a Nivel Nacional de La República Del Ecuador 2026–2035; República del Ecuador: Quito, Ecuador, 2025.
  25. MAATE. Plan Nacional de Adaptación Al Cambio Climático Del Ecuador (2022–2027); MAATE: Quito, Ecuador, 2023. [Google Scholar]
  26. Torres, B.; Herrera-Feijoo, R.; Torres, Y.; García, A. Global Evolution of Research on Silvopastoral Systems through Bibliometric Analysis: Insights from Ecuador. Agronomy 2023, 13, 479. [Google Scholar] [CrossRef] [Scilit]
  27. Griscom, B.W.; Adams, J.; Ellis, P.W.; Houghton, R.A.; Lomax, G.; Miteva, D.A.; Schlesinger, W.H.; Shoch, D.; Siikamäki, J.V.; Smith, P.; et al. Natural Climate Solutions. Proc. Natl. Acad. Sci. USA 2017, 114, 11645–11650. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  28. Garrett, R.; Ferreira, J.; Abramovay, R.; Brandão, J.; Brondizio, E.; Euler, A.; Pinedo, D.; Porro, R.; Cabrera Rocha, E.; Sampaio, O.; et al. Transformative Changes Are Needed to Support Socio-Bioeconomies for People and Ecosystems in the Amazon. Nat. Ecol. Evol. 2024, 8, 1815–1825. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  29. Somarriba, E.; Cerda, R.; Orozco, L.; Cifuentes, M.; Dávila, H.; Espin, T.; Mavisoy, H.; Ávila, G.; Alvarado, E.; Poveda, V.; et al. Carbon Stocks and Cocoa Yields in Agroforestry Systems of Central America. Agric. Ecosyst. Environ. 2013, 173, 46–57. [Google Scholar] [CrossRef] [Scilit]
  30. McGroddy, M.E.; Lerner, A.M.; Burbano, D.V.; Schneider, L.C.; Rudel, T.K. Carbon Stocks in Silvopastoral Systems: A Study from Four Communities in Southeastern Ecuador. Biotropica 2015, 47, 407–415. [Google Scholar] [CrossRef] [Scilit]
  31. Torres, B.; Herrera-Feijoo, R.J.; Torres-Navarrete, A.; Bravo, C.; García, A. Tree Diversity and Its Ecological Importance Value in Silvopastoral Systems: A Study along Elevational Gradients in the Sumaco Biosphere Reserve, Ecuadorian Amazon. Land 2024, 13, 281. [Google Scholar] [CrossRef] [Scilit]
  32. Torres, B.; Bravo, C.; Torres, A.; Tipán-Torres, C.; Vargas, J.C.; Herrera-Feijoo, R.J.; Heredia-R, M.; Barba, C.; García, A. Carbon Stock Assessment in Silvopastoral Systems along an Elevational Gradient: A Study from Cattle Producers in the Sumaco Biosphere Reserve, Ecuadorian Amazon. Sustainability 2023, 15, 449. [Google Scholar] [CrossRef] [Scilit]
  33. Montagnini, F.; Nair, P.K.R. Carbon Sequestration: An Underexploited Environmental Benefit of Agroforestry Systems. Agrofor. Syst. 2004, 61, 281–295. [Google Scholar] [CrossRef] [Scilit]
  34. Schroth, G.; Mota, M.S.S.; Jerozolimski, A. Agroforestry and the Conservation of Forest Cover and Biodiversity in Tropical Landscapes—On-Site and off-Site Effects and Synergies with Environmental Legislation. In Sistemas Agroflorestais—Bases Científicas para o Desenvolvimento Sustentável; Universidade Estadual do Norte Fluminense Darcy Ribeiro: Campos dos Goytacazes, Brazil, 2004; pp. 67–86. [Google Scholar]
  35. Perfecto, I.; Vandermeer, J.; Wright, A. Nature’s Matrix: Linking Agriculture, Biodiversity Conservation and Food Sovereignty; Perfecto, I., Vandermeer, J., Wright, A., Eds.; Earthscan Publications Ltd.: London, UK, 2019; pp. 1–295. [Google Scholar] [CrossRef] [Scilit]
  36. Álava-Núñez, P.; Torres, B.; Castro, M.; Robles, M. AGB Carbon Stock Analysis in the Indigenous Agroforestry of the Ecuadorian Amazon: Chakra and Aja as Natural Climate Solutions. Front. For. Glob. Change 2025, 8, 1513140. [Google Scholar] [CrossRef] [Scilit]
  37. Perreault, T. Why Chacras (Swidden Gardens) Persist: Agrobiodiversity, Food Security, and Cultural Identity in the Ecuadorian Amazon. Hum. Organ. 2005, 64, 327–339. [Google Scholar] [CrossRef] [Scilit]
  38. Coomes, O.T.; Takasaki, Y.; Abizaid, C.; Arroyo-mora, J.P. Environmental and Market Determinants of Economic Orientation among Rain Forest Communities: Evidence from a Large-Scale Survey in Western Amazonia. Ecol. Econ. 2016, 129, 260–271. [Google Scholar] [CrossRef] [Scilit]
  39. Chazdon, R.L.; Brancalion, P.H.S.; Laestadius, L.; Bennett-Curry, A.; Buckingham, K.; Kumar, C.; Moll-Rocek, J.; Vieira, I.C.G.; Wilson, S.J. When Is a Forest a Forest? Forest Concepts and Definitions in the Era of Forest and Landscape Restoration. Ambio 2016, 45, 538–550. [Google Scholar] [CrossRef] [Scilit]
  40. Montagnini, F.; Ibrahim, M.; Restrepo, E.M. Silvopastoral Systems and Climate Change Mitigation in Latin America. Bois For. Des. Trop. 2013, 67, 3–16. [Google Scholar] [CrossRef] [Scilit]
  41. Torres, B.; Günter, S.; Acevedo-Cabra, R.; Knoke, T. Livelihood Strategies, Ethnicity and Rural Income: The Case of Migrant Settlers and Indigenous Populations in the Ecuadorian Amazon. For. Policy Econ. 2018, 86, 22–34. [Google Scholar] [CrossRef] [Scilit]
  42. Berkes, F. Evolution of Co-Management: Role of Knowledge Generation, Bridging Organizations and Social Learning. J. Environ. Manag. 2009, 90, 1692–1702. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  43. Schmitz, M.F.; Herrero-Jáuregui, C. Cultural Landscape Preservation and Social–Ecological Sustainability. Sustainability 2021, 13, 2593. [Google Scholar] [CrossRef] [Scilit]
  44. Chapin, F.S. Transformative Earth Stewardship: Principles for Shaping a Sustainable Future for Nature and Society. Earth Steward. 2024, 1, e12023. [Google Scholar] [CrossRef] [Scilit]
  45. Huntington, J.L.; Hegewisch, K.C.; Daudert, B.; Morton, C.G.; Abatzoglou, J.T.; McEvoy, D.J.; Erickson, T. Climate Engine: Cloud Computing and Visualization of Climate and Remote Sensing Data for Advanced Natural Resource Monitoring and Process Understanding. Bull. Am. Meteorol. Soc. 2017, 98, 2397–2409. [Google Scholar] [CrossRef] [Scilit]
  46. Vera-Vélez, R.; Cota-Sánchez, J.H.; Olmedo, J.E.G. Biodiversity, Dynamics, and Impact of Chakras on the Ecuadorian Amazon. J. Plant Ecol. 2019, 12, 34–44. [Google Scholar] [CrossRef] [Scilit]
  47. Tonucci, R.; Nair, V.; Ramachandran, P.K.; Garcia, R. Grass vs. Tree Origin of Soil Organic Carbon under Different Land-Use Systems in the Brazilian Cerrado. Plant Soil. 2017, 419, 281–292. [Google Scholar] [CrossRef] [Scilit]
  48. Van Breugel, M.; Ransijn, J.; Craven, D.; Bongers, F.; Hall, J.S. Estimating Carbon Stock in Secondary Forests: Decisions and Uncertainties Associated with Allometric Biomass Models. For. Ecol. Manag. 2011, 262, 1648–1657. [Google Scholar] [CrossRef] [Scilit]
  49. Roshetko, J.M.; Lasco, R.D.; Delos Angeles, M.S. Smallholder Agroforestry Systems For Carbon Storage. Mitig. Adapt. Strateg. Glob. Change 2006, 12, 219–242. [Google Scholar] [CrossRef] [Scilit]
  50. Slik, J.W.F. Estimating Species-Specific Wood Density from the Genus Average in Indonesian Trees. J. Trop. Ecol. 2006, 22, 481–482. [Google Scholar] [CrossRef] [Scilit]
  51. Chave, J.; Andalo, C.; Brown, S.; Cairns, M.A.; Chambers, J.Q.; Eamus, D.; Fölster, H.; Fromard, F.; Higuchi, N.; Kira, T.; et al. Tree Allometry and Improved Estimation of Carbon Stocks and Balance in Tropical Forests. Oecologia 2005, 145, 87–99. [Google Scholar] [CrossRef] [Scilit]
  52. Baker, T.R.; Phillips, O.L.; Malhi, Y.; Almeida, S.; Arroyo, L.; Di Fiore, A.; Erwin, T.; Killeen, T.J.; Laurance, S.G.; Laurance, W.F.; et al. Variation in Wood Density Determines Spatial Patterns in Amazonian Forest Biomass. Glob. Change Biol. 2004, 10, 545–562. [Google Scholar] [CrossRef] [Scilit]
  53. Blanc, L.; Echard, M.; Herault, B.; Bonal, D.; Marcon, E.; Baraloto, C.; Chave, J. Dynamics of Aboveground Carbon Stocks in a Selectively Logged Tropical Forest. Ecol. Appl. 2009, 19, 1397–1404. [Google Scholar] [CrossRef] [Scilit]
  54. Chave, J.; Coomes, D.; Jansen, S.; Lewis, S.L.; Swenson, N.G.; Zanne, A.E. Towards a Worldwide Wood Economics Spectrum. Ecol. Lett. 2009, 12, 351–366. [Google Scholar] [CrossRef] [Scilit]
  55. Mokany, K.; Raison, R.J.; Prokushkin, A.S. Critical Analysis of Root: Shoot Ratios in Terrestrial Biomes. Glob. Change Biol. 2006, 12, 84–96. [Google Scholar] [CrossRef] [Scilit]
  56. IPCC. Global Warming of 1.5 °C: An IPCC Special Report on the Impacts of Global Warming of 1.5 °C Above Pre-Industrial Levels and Related Global Greenhouse Gas Emission Pathways, in the Context of Strengthening the Global Response to the Threat of Climate Change; Masson-Delmotte, V.P., Zhai, H.-O., Pörtner, D., Roberts, J., Skea, P.R., Shukla, A., Pirani, W., Moufouma-Okia, C., Péan, R., Pidcock, S., et al., Eds.; Cambridge University Press: Cambridge, UK; New York, NY, USA, 2018. [Google Scholar]
  57. Cairns, M.A.; Brown, S.; Helmer, E.H.; Baumgardner, G.A. Root Biomass Allocation in the World’s Upland Forests. Oecologia 1997, 111, 1–11. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  58. Díaz, S.; Kattge, J.; Cornelissen, J.H.C.; Wright, I.J.; Lavorel, S.; Dray, S.; Reu, B.; Kleyer, M.; Wirth, C.; Colin Prentice, I.; et al. The Global Spectrum of Plant Form and Function. Nature 2016, 529, 167–171. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  59. Cohen, J. Statistical Power Analysis for the Behavioral Sciences Second Edition. J. Am. Stat. Assoc. 1978, 73, 680. [Google Scholar]
  60. Nakagawa, S.; Cuthill, I.C. Effect Size, Confidence Interval and Statistical Significance: A Practical Guide for Biologists. Biol. Rev. 2007, 82, 591–605. [Google Scholar] [CrossRef] [Scilit]
  61. De la Torre, L.; Navarrete, H.; Muriel, P.; Macía, M.J.; Balslev, H. Enciclopedia de las Plantas Útiles del Ecuador; Primera, Ed.; Herbario QCA de la Escuela de Ciencias Biológicas de la Pontificia: Quito, Ecuador, 2008; ISBN 9978771352. [Google Scholar]
  62. Rios, M.; Koziol, M.; Borgtoft, H.; Granda, G. Plantas Útiles Del Ecuador: Aplicaciones, Retos y Perspectivas; Ediciones Abya-Yala: Quito, Ecuador, 2007. [Google Scholar]
  63. Lerner, A.M.; Rudel, T.K.; Schneider, L.C.; McGroddy, M.; Burbano, D.V.; Mena, C.F. The Spontaneous Emergence of Silvo-Pastoral Landscapes in the Ecuadorian Amazon: Patterns and Processes. Reg. Environ. Change 2014, 15, 1421–1431. [Google Scholar] [CrossRef] [Scilit]
  64. Torres, B.; Espinoza, Í.; Torres, A.; Herrera-Feijoo, R.; Luna, M.; García, A. Livelihood Capitals and Opportunity Cost for Grazing Areas’ Restoration: A Sustainable Intensification Strategy in the Ecuadorian Amazon. Animals 2023, 13, 714. [Google Scholar] [CrossRef] [Scilit]
  65. Gliessman, S.R. Nature’s Matrix: Linking Agriculture, Conservation, and Food Sovereignty. BioScience 2011, 61, 77–78. [Google Scholar] [CrossRef] [Scilit]
  66. López-Cubillos, S.; Mason, N.; Wintle, B.; Pacheco, P.; Ochoa-Quintero, J.M.; Nascimento, N.; Torres, B.; Runting, R.K. To Implement the Belém Declaration, We Need a Structured and Collaborative Approach. Proc. Natl. Acad. Sci. USA 2025, 122, 2420198122. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  67. Montagnini, F. La Necesidad de Incentivos Financieros Para Fomentar Los Sistemas Agroforestales Como Islas de Biodiversidad En Paisajes Degradados. Rev. Cienc. Ambient. 2025, 60, 1–11. [Google Scholar] [CrossRef] [Scilit]
  68. Torres, B.; Herrera-Feijoo, R.J.; Cedillo, E.; Robles, M.; Velasco, C. Incentivos Forestales Para La Sostenibilidad: Propuesta Estratégica Hacia Una Cultura Forestal En Ecuador. Horiz. Nexus J. 2025, 3, 84–93. [Google Scholar] [CrossRef] [Scilit]
Figure 1. Study area location and temporary plots established along the land use systems.
Sustainability 18 02451 g001
Figure 2. Monthly temperature and rainfall in the study area (Arosemena Tola, 400–800 m.a.s.l.). Source: authors’ elaboration based on the information available in [45].
Sustainability 18 02451 g002
Figure 3. Visual contrast among the three land-use systems evaluated: (a) agroforestry plot with Theobroma cacao under multi-strata canopy, (b) cattle pasture with remnant timber trees (silvopasture), and (c) remnant primary forest fragment within the Sumaco Biosphere Reserve.
Sustainability 18 02451 g003
Figure 4. Mean above- and below-ground biomass, carbon, and CO2-equivalent stocks (Mg ha−1) across agroforestry, silvopastoral, and forest systems in Arosemena Tola, Ecuador. Bars indicate the contribution of trees, roots, and cocoa/grass components to total values.
Sustainability 18 02451 g004
Figure 5. Aboveground carbon (C) and CO2-equivalent (CO2eq) stocks (Mg ha−1) by dominant tree species across agroforestry, silvopastoral, and forest systems in Arosemena Tola, Ecuador. Bars represent species-level contributions to total carbon stocks within each land-use system. Numbers in parentheses indicate the number of individuals recorded per species.
Sustainability 18 02451 g005
Figure 6. Hierarchical clustering (Bray–Curtis + Ward) of dominant tree species (DBH ≥ 10 cm) across forest, agroforestry, and silvopastoral systems in Arosemena Tola, Ecuador. The three clusters reflect floristic differentiation consistent with land-use type, supporting the role of tree-based production systems as structurally distinct but ecologically connected components of the Andean–Amazonian landscape.
Sustainability 18 02451 g006
Figure 7. Conceptual model of a biocultural productive landscape linking natural forest, cacao-based traditional agroforestry (Amazonian Chakra), and tree-rich traditional silvopastoral systems in the Andean–Amazon region. Circles summarize tree species richness (DBH ≥ 10 cm), tree density (trees ha−1), and mean aboveground carbon stocks expressed as CO2-equivalent (Mg CO2eq ha−1) for each land-use system. Central values indicate the proportion of forest attributes conserved by agroforestry and silvopastoral systems, while bidirectional arrows represent ecological and cultural feedback that sustain tree cover, carbon retention, and livelihood functions across the landscape.
Sustainability 18 02451 g007
Table 1. Comparative overview of conceptual frameworks of human–environment interactions in productive landscapes.
Conceptual FrameworkCore CharacteristicsTerritorial Context/ScaleRelation to BPLs (This Study)Reference
Working LandscapesPromote multifunctionality and connectivity to maintain ecosystem services in productive areas.Agroforestry, pastoral systems, agricultural matrices.BPLs extend this by integrating tree cover maintained through cultural selection and TEK.[10]
Biocultural LandscapesEmphasize co-evolution of cultural identity and ecological processes; focus on TEK.Initially defined for island territories; extended globally.BPLs broaden this by combining biocultural logic with measurable carbon and livelihood functions in forest–production matrices.[11]
Cultural Landscape StewardshipAdvocates for participatory, heritage-based landscape management; critiques exclusionary conservation models.Traditional rural landscapes.BPLs operationalize this through empirical evidence on biodiversity and carbon in managed production systems.[43]
Earth StewardshipCalls for socio-ecological transitions toward ecosystem health + human well-being.Global, territorial, multi-scalar.BPLs act as grounded case studies of stewardship in action, adapted to forest–agriculture mosaics.[44]
Biocultural Productive Landscapes (BPLs) (this study)Tree-based territorial systems where ecological processes, TEK, subsistence, and market production co-exist; retain 20–30% of forest carbon and up to 26% of species richness.Cacao agroforestry and silvopasture in the Andean–Amazon of Ecuador.Introduces an integrated, empirical landscape model absent in previous conceptualizations.This study
Table 2. Mean (±SD) values, ANOVA, and Tukey HSD results for tree density, structural attributes, and diversity indices across agroforestry, silvopastoral and forest systems in Arosemena Tola, Ecuador.
VariableAgroforestry (n = 9)Silvopasture (n = 9)Forest (n = 10)1 p-Value
Tree density (ind ha−1)177.08 ± 104.53 a194.06 ± 112.37 a626.00 ± 117.30 b***
Average DBH (cm)19.15 ± 2.19 a19.37 ± 5.59 b21.96 ± 2.24 bn/s
Basal area (m2 ha−1)5.85 ± 4.28 a7.81 ± 4.44 a30.75 ± 9.16 b***
Species richness (S)6.78 ± 3.34 a9.00 ± 2.55 a26.50 ± 4.22 b***
Family richness7.56 ± 4.61 a7.78 ± 1.98 a18.10 ± 2.92 b***
Shannon index (H′)1.22 ± 0.44 a1.45 ± 0.35 a2.90 ± 0.23 b***
Simpson index (1–D)0.56 ± 0.18 a0.65 ± 0.13 a0.91 ± 0.03 b***
1 p-Value: *** p < 0.001; n/s = nonsignificant. Letters in superscript denote significant differences between land uses.
Table 3. Mean (±SD) values, ANOVA, and Tukey HSD results for tree above- and below-ground biomass and carbon stocks across agroforestry, silvopastoral and forest systems in Arosemena Tola, Ecuador.
VariableAgroforestry (n = 9)Silvopasture (n = 9)Forest (n = 10)1 p-Value
AGBtrees (Mg ha−1)45.93 ± 33.59 a81.35 ± 48.20 a283.86 ± 103.16 b***
AGCtrees (Mg ha−1)21.58 ± 15.78 a37.87 ± 26.68 a133.41 ± 48.48 b***
AGCO2eq_tress (Mg ha−1)79.15 ± 57.89 a140.21 ± 83.07 a489.23 ± 177.80 b***
BGBroots_trees (Mg ha−1)11.73 ± 10.27 a24.40 ± 14.45 a85.15 ± 30.94 b***
BGCroots_trees (Mg ha−1)4.67 ± 4.73 a11.46 ± 6.80 a40.02 ± 14.54 b***
BGCO2eq_roots_tress (Mg ha−1)23.74 ± 17.37 a42.06 ± 24.93 a146.77 ± 53.06 b***
Total tree biomass (Mg ha−1)59.70 ± 43.07 a105.75 ± 65.62 a369.02 ± 134.11 b***
Total tree carbon stock (Mg ha−1)28.06 ± 20.52 a49.26 ± 29.46 a173.44 ± 63.03 b***
Total tree CO2eq stock (Mg ha−1)102.92 ± 75.26 a182.28 ± 107.99 a636.01 ± 231.14 b***
1 p-Value: *** p < 0.001. Letters in superscript denote significant differences between land uses.
Table 4. Tree species actively retained in agroforestry (AFS) and silvopastoral (SPS) systems, showing forest occurrence (ind ≥ 10 cm DBH ha−1), conservation status, and wood density.
RankFamilySpeciesLand UsesLivelihood-Related UseConservation and Functional Attributes
Chakra–AFS Traditional–SPS ForestFood (Human/Animal)MedicinalCultural/Spiritual Material/TimberNative/Non-NativeIUCN CategoryWood Density (g cm−3)
1CordiaceaeCordia alliodora61602xxNLC0.53
2BignoniaceaeJacaranda copaia3325xxNLC0.6
3MirtaceaePsidium guajava144xxxNLC0.71
4FabaceaeInga edulis3313xxxxNLC0.56
5AsteraceaePiptocoma discolor1986xxxNLC0.47
6MelastomataceaeMiconia sp.1722xxxxN0.63
7AsteraceaeVernonanthura patens312xxxNLC0.54
8ArecaceaeBactris gasipaes74xxxxNLC0.42
9MeliaceaeCedrela sp.344xxxxN0.44
10RutaceaeCitrus sinensis92xxxNNLC0.71
11RutaceaeCitrus aurantiifolia6xxxNNLC0.71
12RutaceaeZanthoxylum riedelianum31xxxNLC0.61
13MyristicaceaeOtoba glycycarpa31xxxNDD0.39
14LauraceaePersea americana3xxxxNLC0.6
15AnacardiaceaeSpondias mombin3xxxNLC0.63
16AraliaceaeSchefflera morototoni23xxxxNLC0.44
17BignoniaceaeTabebuia chrysantha21xxNVU1.0
18MalvaceaeTheobroma bicolor1xxxNLC0.61
19AnnonaceaeAnnona sp.1xxxxN0.47
20CecropiaceaePourouma cecropiifolia11xxxNLC0.36
“x” indicates documented use based on de la Torre et al. [61] and Ríos et al. [62]; “–” indicates use not documented. IUCN categories: LC = Least Concern; VU = Vulnerable; DD = Data Deficient. N = native; NN = non-native.
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.