


Abstract
Per- and polyfluoroalkyl substances (PFAS) continue to be one of the most persistent global contaminants and are increasingly recognized as leading metabolic- and hepatic-dysfunction mediators. Despite extensive investigation of PFAS toxicity, a critical gap in the identification and integration of toxicokinetic drivers of hepatic bioaccumulation with mechanistic pathways driving mitochondrial and nuclear receptor-related injury, more specifically, with respect to alternative PFAS strategies, still remains. Legacy PFAS, including PFOA and PFOS, accumulate in the liver and disturb mitochondrial homeostasis as they disrupt β-oxidation, induce oxidative stress, and alter lipid and bile acid metabolism. Meanwhile, the next-generation PFAS variants (including short-chain and polymeric substitutes) are rapidly increasing in environmental concentrations, but remain insufficiently characterized and poorly regulated, raising concerns that substitution-based strategies may maintain their toxicological risk. We summarize the evidence of the association between PFAS bioaccumulation and mitochondrial dysfunction, metabolic reprogramming, and inflammatory signaling, and illustrate mechanistic convergence across legacy and emerging PFAS. We also review insights from recent experimental models, such as 3D hepatocyte systems and human-relevant receptor platforms that more closely mimic chronic exposure states. This review emphasizes mechanistic convergence across legacy and emerging PFAS, highlighting shared pathways that may persist despite chemical substitution. Thus, we discuss key gaps in monitoring, toxicity assessment, and policy, including the requirement of regulatory paradigms that treat PFAS as a class rather than individual compounds.
1. Introduction
Per- and polyfluoroalkyl substances (PFAS), or “forever chemicals”, are synthetic substances widely used in industrial and consumer products. The compounds are found in food packaging, pesticides, firefighting foams, waterproofing products, paints, and cosmetics [1,2]. Environmental studies have shown PFAS buildup in terrestrial and marine systems and processed foods [3,4,5,6,7]. Uptake of PFAS into edible crops grown on biosolids-amended soils is now a well-documented additional dietary pathway [8]. Beer and tea have also emerged as unexpected sources of ultrashort-chain PFAS such as trifluoroacetate [9].
Such broad exposure results in substantial human exposure, primarily through dietary consumption. Since PFAS compounds have caused significant environmental contamination, understanding how they enter the human population is essential for proper health risk assessment. The application of diverse PFAS compounds in food-contact materials is a significant concern. These are applied to food packaging containers and nonstick cookware [10,11]. The transport of PFAS compounds from these materials can be a major route for food contaminants and human exposure through dietary consumption [12,13]. Beyond individuals exposed to these contaminants, some occupational categories are exposed to significantly higher levels. Firefighters, who are constantly exposed to aqueous film-forming foams and industrial workers in fluorochemical manufacturing, have substantially higher PFAS exposures [14,15]. These occupational exposures may help clarify the health impacts of higher PFAS doses, complementing our knowledge from population-level studies.
2. Global Epidemiological Evidence of Widespread PFAS Exposure
Per- and polyfluoroalkyl substances (PFAS) are a public health concern worldwide, and human exposure is reported globally, as on many continents. Biomonitoring data from the United States National Health and Nutrition Examination Survey (NHANES) confirm nearly uniform exposure, with detection rates above 98% of legacy PFAS compounds (PFOS, PFOA, PFHxS, PFNA) in the U.S. general population since 1999 [16,17]. However, over 96% of U.S. adolescents aged 12–19 years have detectable serum concentrations of these legacy compounds [17], despite significant drops in geometric mean concentrations of PFOS (more than 85%) and PFOA (more than 70%) between 1999–2000 and 2017–2020 as industrial phase-outs took place. European biomonitoring using the Human Biomonitoring for Europe (HBM4EU) effort (2017–2022) supports this extensive exposure pattern, with the most common PFOA, PFOS, PFHxS and PFNA detected at above 95% prevalence amongst European teenagers and 14.3% of all adolescents studied exceeding the EFSA health-based guidance value of 6.9 μg/L for the sum of four PFAS, with rates as high as 24% in Northern and Western Europe [18,19]. The same pattern of global and regional exposure is recorded with East Asian populations: detection rates were greater than 99.7% in five of the most prevalent PFAS evaluated by South Korea’s National Biomonitoring Programme (KoNEHS cycle 4, 2018–2020), and geometric mean serum PFOS concentrations were 15.1 μg/L in adults and 7.97 μg/L in adolescents, which are larger compared to those of contemporary North American and European populations [20]. Biomonitoring studies in Japan suggest elevated exposure to PFAS (16.1–43.5 ng/mL total PFAS) in contaminated spaces near military bases and fluorochemical sites used in production, which indicate significant populations exposed to the PFAS based on established risk assessment guidelines [21]. High-exposure populations located in the vicinity of areas near industrial point sources bear tremendous burdens: communities closer to AFFF-contaminated sites near U.S. military installations had concentrations of serum PFOS, PFOA, and PFHxS 2–10 times higher than national reference levels years after drinking water exposures were remediated [17]. Furthermore, European data on occupational exposures showed heightened contamination levels in chrome plating facility workers and surrounding fluorochemical manufacturing hotspots with exceedance rates as high as 23.8% higher than health-based guidance values [19]. Collectively, this epidemiological data creates accumulating proof that PFAS exposure is nearly ubiquitous among industrialized populations and persistence of legacy compounds are still far above the endpoint levels even in the face of regulation phaseouts, regional discrepancy in intensity of exposure relative to the industrial production and source of contamination associated with PFAS exposures and heavy reliance of exposure within occupationally exposed populations and populations, and that exposure in communities adjacent to point-source sources of contamination with a large impact.
Dietary patterns and food consumption habits are also among the primary contributors to the PFAS exposure profile of most individuals [22,23,24,25,26]. Serum PFAS concentrations varied widely by sex, with higher levels in men than in women [18,27,28]. Among studies focusing on PFAS elimination in females, biological factors, such as menstruation and breastfeeding, were associated with lower serum concentrations [28,29,30,31,32,33]. The worldwide increase in PFAS detection in dairy products and infant formula has raised questions about child exposure risks [7,34,35]. Monitoring PFAS levels in pregnant women is now essential for identifying effective methods to reduce potential exposures and for implementing prevention or intervention programs. Human autopsy studies consistently show the highest PFAS concentrations in the liver, kidneys, lungs, brain, and bone with clear chain-length-dependent patterns [36,37]. Due to their environmental persistence and bioaccumulation, which are critical for human health, and the widespread human exposure to PFAS compounds, their toxic mechanisms must be understood [38,39,40]. The liver is a primary target organ affected by PFAS, while mitochondria are particularly sensitive to PFAS exposure. This review will discuss PFAS-induced alterations in cellular and molecular mechanisms, including mitochondrial function, that lead to liver damage in exposed individuals.
While previous reviews presented PFAS toxicity within the wider context or targeted specific endpoints (e.g., reproductive toxicity, immunotoxicity, or environmental fate), our review gives a complementary and integrated perspective on hepatic toxicity mechanisms. We present a synthesis of recent progress on three major topics: (1) the mechanistic elucidation of PFAS bioaccumulation via protein–phospholipid interactions as opposed to classical lipid partitioning, (2) the data from high-tech 3D cellular models combined with in vivo and epidemiological evidence to link experimental and human health impacts, and (3) the reconciliation of perceived discrepancies in cholesterol metabolism using context-specific and receptor-dependent perspectives. We also highlighted the recent literature (2022–2025) that focuses on environmentally relevant exposure levels and chronic exposure models, addressing the limitations of previous high-dose acute toxicity studies.
3. Toxicokinetics and Bioaccumulation
Understanding how PFAS compounds enter the body and distribute through other organs is fundamental to understanding their toxic effects [36,37,41]. PFAS may be absorbed by the intestine when ingested through food. In rats, absorption rates of PFAS compounds can reach 100%, indicating efficient absorption by the digestive system. Indeed, large-scale animal studies demonstrate that the vast majority have absorption rates exceeding 95% and rapid gut absorption of PFAS compounds [36,41,42,43,44,45,46]. Near-complete oral absorption of PFBS, PFHxS, and PFOS has been confirmed in both sexes of Sprague-Dawley rats [44]. Dairy cows fed naturally contaminated feed rapidly secrete PFBSs, PFHxS, PFOS, and PFOA into milk [47], suggesting efficient hepatic uptake based on the ability of organic anion-transporting polypeptides (OATPs, particularly OATP1B1 and OATP1B3) [45,48] and sodium taurocholate cotransporting polypeptide (NTCP) [49], resulting in active secretory transport to milk. Such inactivation is accompanied by enterohepatic recirculation, in which PFAS are secreted in bile through efflux transporters and subsequently reabsorbed by specific uptake transporters into the intestine [50]. Portal-mediated uptake of PFAS by intestinal epithelium exploits channels typically involved in bile acid recirculation, including (1) the intestinal uptake (i.e., OATP2B1) (apical membrane) [48] and functional apical sodium-dependent bile acid transporter (ASBT) mediating active absorption from intestinal lumen [49], (2) the hepatic uptake (i.e., OATP1B1, OATP1B3 [48] and NTCP [49]) mediating an efficient extraction from portal blood into hepatocytes, (3) the renal transporters (i.e., OAT1, OAT3 (basolateral secretion) and OAT4 [51], URAT1 (apical reabsorption)) modulate urinary excretion, and, finally, (4) the amphiphilic nature of PFAS (characterized by perfluorinated carbon chains and acidic head groups) presents high-affinity binding to the organic anion transporters that evolved for endogenous bile acids and organic anions.
After absorption, detailed studies have shown how PFAS compounds cross the intestinal barrier into systemic circulation, bind to circulating proteins, including albumin and low-density lipoprotein, and distribute to extraintestinal organs via the blood [36,37,41,42,52]. Greater than 99% of PFAS components are associated with serum proteins [53]. Such extensive protein binding has profound implications for distribution and elimination kinetics. The structure–activity relationships for the binding selectivity of PFAS compounds to plasma proteins are established. PFAS with carbon chain lengths of seven or more carbon atoms have a higher binding affinity for globulins than short-chain PFAS, which selectively bind to albumin [53]. This selective binding of human serum proteins increases the likelihood of distribution to tissues and the extracellular plasma [54]. In addition, PFAS molecules preferentially bind to cellular phospholipids, which has a marked influence on tissue distribution, especially for longer-chain PFAS [54]. These binding properties play a direct role in determining organ-specific accumulation patterns for PAFS, which accumulate with the highest concentrations in the liver, kidneys, and lungs [36,55,56,57,58,59]. Due to the high protein-binding affinity of these compounds, the protein-rich hepatic tissue makes the liver the primary site of PFAS accumulation [40,59,60]. Per- and polyfluoroalkyl substances (PFAS) demonstrate widespread bioaccumulation in biota and the environment owing to their persistent chemical structures. Traditional bioaccumulation metrics, such as octanol–water partition coefficients (KOW), are used extensively for hydrophobic organic contaminants but are of limited predictive value for PFAS because of their amphiphilic structure and strong affinity for proteins and phospholipids rather than neutral lipids. Meta-analysis of published bioconcentration factors (BCFs) and bioaccumulation factors (BAFs) shows that for aquatic species, legacy PFAS such as perfluorooctane sulfonic acid (PFOS) and perfluorooctanoic acid (PFOA) exhibit substantial accumulation in whole-body tissues, with median log BAF values of 3.55 and 2.16, respectively, in fish, underscoring their capacity to partition into organisms relative to water exposure levels [61]. In Pimephales promelas (fathead minnows), controlled uptake experiments show that accumulation is chain-length-dependent and that both tissue and plasma concentrations of longer-chain perfluoroalkyl carboxylic acids (PFCAs) and sulfonates (PFSAs) increase, with steady-state BAFs up to 26.6 L kg−1 for PFOA, and blood–water partitioning coefficients (PBW) as high as 85.8, indicating preferential PFAS partitioning into biotic phases relative to water [62]. In terrestrial plants, PFAS uptake is predominantly via root absorption from soil, where longer-chain PFAS are preferentially retained in root tissues and yield higher bioaccumulation factors when expressed across plant organs; shorter-chain PFAS distribute more readily to aboveground tissues [8]. In vitro partitioning studies demonstrate that PFAS partition into biological compartments is driven by specific affinities for proteins (e.g., human serum albumin) and phospholipid membranes rather than classical hydrophobicity (log KOW), with protein–water distribution coefficients often exceeding membrane partitioning at lower exposure concentrations [63,64]. Long-chain PFAS, including PFOS and PFOA, have higher bioaccumulation potential than short-chain analogs [61,62], and despite low KOW values, can surpass regulatory limits. These protein–water and membrane–water partition coefficients provide biologically relevant analogs to KOW and help explain how PFAS bioaccumulate despite weak neutral lipid partitioning, making experimentally derived BCFs, BAFs, and biological phase partition coefficients more accurate descriptors of PFAS bioaccumulation behavior [64].
In vivo studies reveal that PFAS distribution is primarily influenced by the structure of their carbon chains. Short-chain PFAS compounds accumulate in certain organs on a localized scale, while long-chain PFAS compounds are found more evenly throughout the body [65]. Also, species, sex, and the administered dose level strongly influence PFAS chemical distribution [65]. This distribution is important to understand for determining the different levels of toxicity of PFAS compounds.
PFAS compounds break down slowly because of their strong carbon–fluorine bonds [66,67]. Their half-life in biological systems is directly linked to their carbon chain length. Short-chain variants last for hours; longer chains last for years or even decades [41,65,68]. Machine learning models predict median human half-lives of several years for C8–C11 PFCAs/PFSAs and much shorter durations for short-chain compounds [69]. At the ecosystem level, environmental and food-web studies further demonstrate that PFAS bioaccumulation occurs across trophic levels, with measured bioaccumulation factors in plants, invertebrates, and fish supporting chain-length-dependent accumulation and trophic magnification for several long-chain PFAS [8,70]. These findings support mammalian toxicokinetic data by providing quantitative accumulation metrics across biological systems.
Similarly, biological sex and species differences also play important roles in the elimination half-lives of PFAS compounds [36,71,72]. In a previous study, Dzierlenga et al. found that female rats have shorter elimination half-lives for PFOA and perfluorohexanoic acid (PFHxA) than male counterparts, suggesting that PFAS clearance from the body may be sex-dependent [71]. Chang et al. also reported that perfluorobutanoic acid (PFBA) removal was faster in rats than in mice, suggesting interspecies variability regarding the toxicokinetics of these compounds [36,72]. Nevertheless, both studies used only rodent models of PFAS metabolism, which may not be representative of human PFAS metabolism, given differences in renal transporter levels across species. This limitation significantly widens the existing knowledge deficit and limits the ability to evaluate human health hazards.
There is a big knowledge gap related to novel PFAS groups, raising doubts about the unique metabolic behavior and persistence profiles of new PFAS subtypes, which are not well characterized [73], because most studies have centered on classical perfluorocarboxylic acids or PFCAs and perfluorosulfonic acids [66]. These new PFAS compounds raise questions about elimination kinetics regarding their biotransformation and metabolite production. The biochemical transformations of PFAS precursor compounds and intermediate metabolites are particularly important in biological systems [36]. Fluorotelomer alcohols (FTOHs) and polyfluoroalkyl phosphate esters are volatile precursors of PFOA compounds that can undergo metabolism in humans to yield PFOA and other PFCA compounds [36]. Similarly, several precursors and intermediates of PFOSs (perfluorooctane sulfonamidoethanols or perfluorooctane sulfonamidoacetic acid) undergo biochemical conversion, which ultimately contributes to total PFOS levels in biological systems [36,74,75].
The transformation of PFAS precursors and intermediates is facilitated by various cytochrome P450 (CYP) isoforms, including variants CYP2A6, CYP2C9, the CYP2C19 isoform, and others in human liver microsomes [74,75], though the molecular mechanisms responsible for these transformations are still insufficiently characterized. A striking observation is the lack of successful biotransformation mechanisms for removing terminal PFAS compounds in humans or other mammalian populations [76,77]. PFAS products are excreted from biological systems through limited routes, leading to their persistence. PFAS compounds are excreted mostly in urine and through bile, breast milk, and menstruation [76]. However, their involvement in enterohepatic circulation pathways has led to particularly limited biliary elimination of PFAS’ age [76]. The enterohepatic circulation process, driven by bile acid reabsorption, returns PFAS compounds to the intestinal system and re-enters liver tissues, thereby contributing to persistent increases in PFAS concentration within the liver [50]. Additionally, PFAS bind to serum albumin and globulin proteins results in urinary excretion rates of less than 0.1%, indicating that filtered PFAS compounds undergo considerable reabsorption in renal tubular structures [53,76]. This highly efficient reabsorption mechanism preserves PFAS compounds in the body, possibly responsible for their markedly extended elimination half-lives and potential for bioaccumulation [77,78]. More generally, rodent models highlight the underlying mechanisms, though human-relevant systems require more detailed applications. Potentially, advanced in vitro liver models or human pharmacokinetic studies are needed to address important gaps in PFAS elimination data. The high absorption efficiency, strong protein binding, metabolism resistance, and extensive renal reabsorption result in a toxicokinetic profile characterized by long-term accumulation and continued exposure in target organs, including the liver [36,41,50,53,77,79].
4. Major Toxic Manifestations of PFAS
Prolonged exposure to PFAS in contaminated in vitro systems, animal models, and human populations has established its association with unfavorable hepatic outcomes. Together, PFAS hepatotoxicity presents in three interrelated areas: structural hepatic injury, lipid and bile acid imbalance, and a wider metabolic alteration with glucose and energy homeostasis (Figure 1). These toxic side effects are hepatomegaly, steatosis, hepatic fibrosis, cholestasis, oxidative stress, and hepatocellular apoptosis. Cellular, in vivo, and epidemiological studies suggest PFAS-induced liver damage depends on the structure of PFAS, duration, and dose of exposure. Indeed, hepatotoxicity is associated with toxic responses to PFAS in various organ systems, most significantly the kidneys, liver, and endocrine systems [80,81,82,83], and the liver remains the most prevalent organ system, contributing significantly to xenobiotic metabolism and hepatic bioaccumulation of PFAS molecules [80,81,82,83]. Hepatotoxic effects of PFAS compounds can occur via hepatomegaly and inflammation, oxidative stress induction, apoptosis, bile acid metabolism disruption, and diverse lipid metabolism variations. In vivo cholestatic liver injury, due to bile acid synthesis and transport being disrupted, was demonstrated to be a clinically relevant phenotypic outcome of PFAS-induced hepatotoxicity [36,75,84,85].
Figure 1.
PFAS exposure and hepatic metabolic disruption: schematic representation of the pathways through which environmental and consumer PFAS exposure can impact liver health. The diagram illustrates how PFAS may induce cellular stress (such as ER stress) and undergo metabolic biotransformation, leading to the disruption of bile acid homeostasis and the formation of persistent metabolites.
Previous epidemiological studies have reported associations with human serum PFAS concentrations and obesity prevalence [81,82,83], suggesting linkage of metabolic dysregulations observed in cell models with population health status. While similar population-level findings do not establish direct causality, the consistency of these data across cohorts supports a meaningful association between PFAS exposure and metabolic dysfunction consistent with experimental observations [81,82,83]. Disruption of hepatic lipid handling is a primary and consistently observed outcome of PFAS exposure among these outcomes. Studies of fatty liver development in response to PFAS exposure have been time- and dose-dependent [86,87,88]. For instance, PFOS has been demonstrated to modulate in vitro specific target genes that encode fatty acid transporters and, in turn, trigger time- and dose-dependent changes in liver fat deposition [86,87,88,89]. Because hepatic lipids are intimately connected to glucose regulation, PFAS-induced disturbance in liver lipid homeostasis often touches on glucose as well. The molecular basis of lipid metabolism disturbance is linked to the increasing incidence of liver disease observed in human populations. The metabolic disruption in PFAS is a matter of closely linked processes that are responsible for glucose metabolism, linking cellular processes directly with a myriad of health consequences. For example, it has been shown that exposure to PFOA significantly elevates fasting blood glucose [90], and it decreases hepatic glycogen and glucose content. These disturbances are mainly determined in the context of metabolic adjustments, which are mediated by enhanced gluconeogenesis and glycogenolysis, and PFAS components have also been found to have functional activities in lipid and liver metabolism in general [91]. The intricate metabolic effects that PFAS exert on glucose metabolism are evident only when new PFAS have been analyzed. In particular, glucose concentrations were elevated in liver tissue after treatment with perfluoro-3,5,7,9-tetraoxadecanoic acid (PFO4DA) or perfluoro-3,5,7,9,11-pentaoxadodecanoic acid (PFO5DoDA) for 140 days. Notably, the serum glucose of the PFO5DoDA-treated group only showed significant increments [92]. This implies that structurally similar PFAS compounds may possess different effects on glucose homeostasis, emphasizing the complex structure–toxicity relationship of PFAS. Exposures, structures, and concentrations of PFAS impact the effects with respect to cell viability, lipid metabolism, bile acid metabolism, glucose metabolism, and amino acid metabolism of hepatocyte cells in many conditions and cell types. These interactions in cellular metabolism characterize the wide range of hepatic pathologies present with PFAS in human beings. These toxic manifestations collectively provide the phenotypic context of our understanding for the interpretation of mechanistic and model-based studies that are examining the molecular and cellular mechanisms where PFAS disrupt hepatic function.
5. Major Molecular Mechanisms
The health effects of PFAS are connected to complex pathways that are important metabolic processes. Understanding these interactions is critical to assessing how PFAS can interfere with normal body functions and be deleterious to health. Nuclear receptors have been identified as the main targets of PFAS compounds, according to researchers. Studies using rodent models indicate that PFOS and PFOA modulate distinct nuclear receptors, thereby promoting the expression of genes involved in metabolism, detoxification, and homeostasis. As one of these targets, the peroxisome proliferator-activated receptor alpha (PPARα) is a key regulator of fatty acid oxidation and lipid homeostasis, which means that its perturbation is particularly important for liver function (Figure 2).
Figure 2.
Mechanism of PFAS-induced metabolic toxicity: proposed adverse outcome pathway (AOP) for PFAS-induced metabolic dysfunction. The figure highlights the progression from an initial molecular event (MIE), such as nuclear receptor activation, to downstream effects including peroxisomal oxidative stress, mitochondrial impairment, and altered lipid metabolism. These collective changes result in a state of oxidative stress and time-dependent metabolic reprogramming.
PFOS, PFOA, and PFBS can indirectly inhibit gene expression in sterol regulatory element-binding protein (SREBP) pathways [78,93,94], underscoring the broad impact of PFAS compounds on metabolic regulation. Multiple human nuclear receptors (PPARα, PPARγ, CAR, PXR, FXR, LXR) are directly activated by both legacy and replacement PFAS in reporter-gene and primary hepatocyte assays [95,96,97]. Transcriptomic dissection of PFOA-exposed mouse liver confirms that the gene signature is driven predominantly by PPARα and CAR activation [96]. Hepatocyte nuclear factor 4α (HNF4α), a major regulator of lipid metabolism, is therefore of particular interest for research [95,98]. The effect of PFOA in human hepatoma cells was shown to inhibit HNF4α expression in human hepatoma cultures through pathways unrelated to PPARα [99]. These findings suggest that PFAS compounds may affect metabolic homeostasis through multiple pathways and may exert additive or synergistic effects.
PFAS interactions with nuclear receptors are not limited to simple agonist or antagonist effects. Louisse and colleagues demonstrated that PFOA, PFOS, and PFNA modified PPARα pathway expression and triglyceride levels in HepaRG cells [100]. Moreover, research by Behr and co-workers demonstrated that, although PFOA and PFOS did not alter cholesterol levels under their experimental conditions, they did remarkably enhance the biosynthesis, metabolism, and transport of bile acids in HepaRG cells [95]. Further investigation of PFAS compounds also indicated notable inhibition of CYP7A1, a regulatory enzyme for the synthesis of bile acids from cholesterol, and increased bile canaliculi dilation in well-differentiated HepaRG cells due to PFAS compound exposure [95]. Impaired regulation of bile acid homeostasis affects lipid metabolism and the rest of the liver, linking nuclear receptor modulation to organ-level effects. The interruption of diverse nuclear receptor networks dysregulating metabolic pathways causes significant alterations in lipid, energy and bile metabolism in the liver after PFAS exposures, producing systemic involvement of pathogenic effects that contribute to hepatotoxicity consistent with observations in both experimental studies and human studies [36,96,101,102,103,104].
PFAS compounds cause liver damage through multiple interconnected molecular pathways, particularly by disrupting nuclear receptors. These overlapping mechanisms work together to trigger significant liver diseases. Understanding how these molecular-level disruptions translate into actual tissue damage helps explain the connection between PFAS exposure and liver injury. Research efforts have demonstrated links between the levels of PFAS and the onset of various liver conditions, such as nonalcoholic fatty liver disease (NAFLD), liver fibrosis, and cancer. Briefly, associations between perfluorononanoic acid (PFNA) compounds and PFOA and NAFLD development, particularly among women and older adults, have been suggested [105,106]. Consistent with these epidemiological findings, extensive research has also examined the associations between PFAS exposure, liver fibrosis development, and cancer initiation [59,107,108]. The epidemiology highlights structure–activity relationships associated with hepatotoxicity, with different PFAS compounds showing varying patterns of liver effects. PFAS exposure, particularly PFOS exposure, was found to have relatively stronger statistical associations with hepatic fibrosis progression than steatosis development [109]. This suggests that PFAS compounds may have differential targets for liver disturbances, perhaps through unique molecular mechanisms.
Recent studies show detrimental impacts of PFAS toxicological effects on the liver in laboratory cellular models, as well as various experimental animal studies performed in diverse research environments [110,111,112,113]. PFAS’s toxic effects on liver cells are associated with concentration, carbon chain structure, molecular properties, and compound interactions [111,112]. Wen and colleagues showed that PFOA and heptafluoropropoxy propanoate (HFPO-DA) exert dose-dependent toxic effects in HepG2 cell cultures, predominantly at lower concentrations and after prolonged exposure [112].
Studies investigating chain length effects reinforce the connection between structure and activity in PFAS-related liver toxicity. Ojo et al. found a significant correlation between PFAS chain length and hepatotoxic potential, with longer PFAS chains demonstrating greater toxicity. This relationship, however, was predominantly based on controlled laboratory models and may not be accurate for whole organisms that may use many different metabolic and compensatory pathways [111]. Hence, the extent to which these data may be applicable to human health risk assessments should be carefully evaluated, particularly based on variations in PFAS-binding proteins and metabolism across species. The complexities of PFAS-related liver toxicity extend beyond individual compound effects; the potential interactions between PFAS constituents also add complexity. When combined with other PFAS, particularly PFOA [111,114], it causes additional toxic effects. These cumulative effects are often greater than a single exposure to individual PFAS compounds, which shows that exposure to several PFAS compounds in the environment might carry more risk than single-compound studies would indicate.
These hepatotoxic effects through molecular pathways are intimately related to the nuclear receptor disturbances described earlier. When the peroxisome proliferator-activated receptor alpha (PPARα) pathway is interrupted, hepatic lipid metabolism is fundamentally altered [81,95,100,115]. The direct association between molecular targets and metabolic dysfunction has also been demonstrated by Louisse and colleagues, who reported that PFOA, PFOS, and PFNA remarkably changed the gene expression of the PPARα pathway and increased triglyceride levels in HepaRG cells [51]. The disturbance of bile acid homeostasis is also another important pathway connecting molecular effects to tissue pathological states. For instance, one study demonstrated that while PFOA and PFOS did not increase cholesterol content, they did markedly enhance the production, metabolism, and transport of bile acids in HepaRG cells [95]. Table 1 summarizes the primary molecular targets affected by PFAS exposure, their physiological roles, the toxic outcomes resulting from their disruption, and supporting references from the reviewed literature.
Table 1.
Key Molecular Targets, Roles, and Associated Toxic Outcomes of PFAS.
6. Advanced Cellular Models and In Vivo Hepatotoxic Effects
In recent years, scientists have been utilizing more complex experimental approaches in order to elucidate the hepatotoxic mechanisms identified in preclinical and clinical settings. Such advanced models are particularly valuable for integrating chronic exposure, multi-pathway disruption, and tissue-level responses that cannot be fully captured by isolated molecular or short-term experimental approaches [84,116]. These complex models provide critical insight into how disruptions in nuclear receptors and modifications in metabolic pathways give rise to tissue-level failures. Especially, 3D hepatocyte culture models have gained traction to investigate the multifaceted effects of PFAS compounds on liver metabolism. These systems address limitations of conventional monolayer cultures by preserving metabolic zonation, prolonged exposure responses, and intercellular signaling relevant to chronic PFAS toxicity. They also more closely resemble Zhang, and others established different metabolite profiles for advanced 3D L-02 cell spheroids exposed to PFOA for 4 or 10 days. Results showed a significant pattern change in six major amino acids for PFOA exposure in the L-02 spheroids after 10 days, but no detectable change after only 4 days of exposure [116]. The time-dependent response pattern highlights the role of exposure duration in PFAS toxicity. Studies focused on short-term exposure may not reveal the complete metabolic effects. Notably, they also showed that the inhibition of glutamine metabolism pathways diminished glutathione (GSH) production and increased oxidative stress in the L-02 spheroids [116]. The greater complexity of 3D culture models has highlighted vital distinctions in the hepatotoxic potential of various PFAS compounds. Hepatotoxicity comparison of PFOA and hexafluoropropylene oxide trimer acid (HFPO-TA) in advanced 3D primary cell spheroids showed that HFPO-TA exhibited significantly increased hepatotoxic potential [84]. The same study also demonstrated that long-term exposure of primary mouse liver spheroids to the PFOA replacement HFPO-TA profoundly disrupts bile acid homeostasis and induces cholestatic injury [84]. This greater toxicity was characterized by decreased cell viability, increased inflammation, reduced albumin and urea production, and significant disruption of cholesterol metabolism pathways [84]. This metabolic and cellular observation is supported and developed in whole-organism studies that demonstrate the biological importance of the observed molecular and cellular effects. Findings from advanced model systems have also reinforced mechanistic observations reported in earlier in vivo and epidemiological studies. The role of the PPARα protein as a primary molecular target of PFAS-induced lipid metabolism disruption has been well described throughout the literature [81,115,117], suggesting a mechanistic connection between lipid microenvironmental observations and molecular/whole-organism metabolic influences. Attema and co-workers reported that HFPO-DA and PFOA enhanced lipids in the liver through the PPARα pathway, and in PPARα-deficient mice, lipid levels were much lower [96]. This finding demonstrated the central role os PPARα in PFAS-related hepatic lipid accumulation. Nevertheless, despite their increased physiological relevance, advanced cellular and animal models remain limited by species-specific metabolic differences and the absence of fully integrated endocrine and immune signaling, underscoring the need for cautious extrapolation to human health outcomes [80,81,115,117]. Table 2 provides a comprehensive overview of experimental model systems used to study PFAS hepatotoxicity, including the compounds tested, key experimental findings, mechanistic insights gained, and relevant citations.
Table 2.
Advanced Cellular Models and In Vivo Studies.
7. Species Differences and Clinical Relevance
Mechanistic understanding from laboratory studies to human health needs to consider that species metabolize, distribute, and respond to PFAS very differently. These differences extend beyond academic interest and directly influence risk assessment and regulatory interventions. The most dramatic instance of this variation between species is observed in cholesterol metabolism, which relates directly to the nuclear receptor pathways identified above. PFAS levels correlate positively with total cholesterol concentrations in human populations [87]. In laboratory mouse models, PFAS exposure has been reported to produce variable effects on cholesterol metabolism, including both increases and decreases in serum cholesterol, dependent on dose, exposure duration, and receptor context [96,118]. This apparent divergence between human and animal responses initially complicated toxicological interpretations. However, emerging evidence suggests that these differences reflect context-dependent biological responses rather than a fundamental contradiction between species [118]. Furthermore, clarifying this contradiction shows that different species express signals from different nuclear receptors differently. The PPARα pathway has been found in many studies to be an important mechanism that mediates PFAS toxicity. Indeed, serum levels of PPARα in mice can be about ten times higher than in humans, indicating that the reported cholesterol level differences are species-specific, due to the fact that cells expressing these receptors differ in major components of PFAS action [125]. Recent studies demonstrate that downregulation does not universally characterize cholesterol responses in mice. Under chronic, steady-state PFOA exposure conditions at environmentally relevant doses, serum and hepatic cholesterol levels increased in a PPARα-dependent manner [118]. This is in contradiction to previous studies, which primarily found decreases in cholesterol levels under high-dose or acute exposure conditions [96]. This suggests that the downregulation of cholesterol is not a universal response to PFAS exposure in mice, but rather a reflection of specific physiological and environmental conditions.
Such mechanistic insights were corroborated by work with genetically modified animal models that closely resemble human receptor expression profiles. In previous work by Schlezinger and others, researchers observed substantial changes in serum cholesterol for PFOA in PFOA-exposed PPARα-humanized mice, which provides evidence for the association between PPARα expression patterns and species response to PFOA [86,118]. This suggests that while the basic toxicity mechanisms are similar between species, the direction and severity of effects may differ because of differences in receptor expression and metabolic pathways after PFAS exposures.
What makes these mechanistic insights particularly valuable for clinical practice is that they are backed up by studies measuring biomarkers of liver and bile acid metabolism. A study reported cholestasis assessed by increased activity of serum gamma-glutamyl transpeptidase (GGT), higher cholesterol and bile acid levels, and elevated liver risk factors in mice after exposure to a blend of five PFAS: PFOS, PFHxS, PFOA, PFNA, and HFPO-DA [85]. These in vivo observations are similar to those seen in human studies and merit the clinical significance of mechanistic investigations. Indeed, a study by Guo et al. found that PFAS exposure caused alterations in mRNA and protein expression of enzymes that are essential in liver bile acid metabolism, through extensive RNA sequencing as well as Western blot analysis [110]. The consistency in these molecular alterations between different experimental conditions and their relationship with human analog biomarkers emphasizes the clinical significance and implications of what has been observed.
Species differences extend beyond endpoint comparisons, involving key aspects of PFAS toxicokinetic characteristics. PFAS compound distribution is strongly affected by species, biological sex, and dosage parameters of compound exposure [65]. These differences have a direct bearing on the intensity of response and timing of effects; they also affect species sensitivity to various PFAS compounds. Understanding these species differences is critically important to interpret toxicological data and include them in risk analysis for human health. The mechanisms of PFAS toxicity show similarities among species, but quantitative responses vary significantly. Thus, mechanistic data from animal models could significantly help however human relevant exposures have to be conducted and taking into consideration while making regulatory decisions.
8. Function Impairment and Energy Metabolism
It is widely acknowledged that the dysregulated cellular energy metabolism is a key mechanism involved in the detrimental hepatic effects of PFAS compounds. Liver depends on mitochondria for β-oxidation of fatty acids, oxidative phosphorylation for ATP, and maintenance of redox homeostasis. Exposure to PFAS drastically disrupts these processes, leading to a cascade of energy shortages and oxidative injury, causing development into clinical liver diseases such as non-alcoholic fatty liver disease (NAFLD)/metabolic-dysfunction-associated steatotic liver disease (MASLD). Impaired fatty acid β-oxidation (the major mitochondrial route for lipid-derived energy) provides the most unequivocal evidence of PFAS-induced mitochondrial dysfunction. Occupational workers with high exposure to PFAS are also shown to exhibit clear β-oxidation abnormalities, with PFOS emerging as the predominant compound in metabolomics [126]. As such, incompletely oxidized fatty acids, decreased ATP production, and the cell’s energy crisis ensue [126]. In bacterial models (as a proxy for conserved mechanisms), PFOS and PFOA are able to induce membrane disruption, a significant amount of reactive oxygen species (ROS) production, and DNA damage, hence proving that basic mitochondrial toxicity pathways are conserved between species [127]. PFAS induce excessive mitochondrial ROS production, surpassing antioxidant mechanisms, including glutathione and superoxide dismutase. The oxidative stress induces lipid peroxidation, protein carbonylation, and mitochondrial DNA damage in hepatocytes [127,128,129]. This imbalance in redox responses is chain-length dependent: those longer-chain PFAS (C8-C11) are more effectively damaging to mitochondrial membrane potential and electron transport chain efficacy than the shorter-chain compounds; however, some shorter-chain compounds tend to elicit compensatory responses in some models [69]. Bioenergetic collapse is also prominent. PFAS uncouple oxidative phosphorylation, attenuate the proton gradient, inhibit mitochondrial biogenesis, and alter the mitochondrial dynamics (fusion/fission balance). PFAS mixtures induce endoplasmic reticulum stress in human liver spheroids and primary hepatocytes by activating unfolded protein response (UPR), which in turn leads to membrane contraction, mitochondria atrophy, and apoptosis [84]. PFOS specifically affects mitochondrial calcium and iron homeostasis, which drives hepatic insulin resistance, which is an important link between mitochondrial failure and metabolic disease [128,129]. The mitochondrial defects directly play a role in the progression of NAFLD/MASLD, which can be listed as follows: (1) Steatosis is due to inhibition of β-oxidation and modification of lipid handling. (2) Steatohepatitis is the by-product of ROS-induced inflammation and Kupffer cell activation. (3) Chronic oxidative injury and pro-oncogenic signaling encourage fibrosis and carcinogenesis [105,106,130]. Other emerging PFAS seem as potent or even more potent in causing mitochondrial toxicity. One such example is HFPO-TA (a GenX processing aid), which significantly disturbs bile acid homeostasis and induces cholestatic damage in 3D mouse liver spheroids by mitochondrial pathways [84]. These mitochondrial disruptions do not occur in isolation as they translate directly to organism-level metabolic disease. In childhood, mitochondrial-mediated lipid dysregulation has been associated with short-chain PFAS (e.g., PFHpA) [124], associated with MASLD in children. The role of glucose homeostasis only emphasizes that mitochondrial dysfunction is connected with global metabolic dysfunction. PFOS exposure disrupts cholesterol and triglyceride homeostasis in the blood circulation [99], affecting whole-body energy metabolism that contributes to high risk for cardiovascular diseases and type 2 diabetes [108,131]. PFOS attaches to hepatic nuclear receptors, resulting in lipid and fatty acid metabolism and related measures of hepatic injury [96]. These hepatic effects stem from widespread perturbations of glucose homeostasis and perturbations in critical energy substrates like amino acids and purines [108,132]. Mitochondrial dysfunction not only impedes energy production but also negatively affects antioxidant defenders and programmed cell death regulation. Disturbances of iron and calcium concentration, specifically in liver mitochondria, are expected to lead to insulin resistance, and excess oxidative stress and apoptosis limit cellular maturation [128,129,133,134,135]. Placental trophoblast studies have also shown PFOS decreases mitochondrial abundance and activity, both of which support preeclampsia and emphasize the developmental role of the mechanism in more general terms [136,137]. The mitochondrial dysfunction associated with PFAS hepatotoxicity can be viewed as potentially the most convergent multiplier pathway that synergistically combines nuclear receptor dysfunction [96], oxidative stress, lipid deposition, and inflammation to promote PFAS hepatotoxicity. It offers a mechanistic conduit between molecular initiating events and clinical liver disease, and explains what low-level chronic exposure looks like, leading to major long-term risk.
9. Emerging PFAS Compounds and Future Health Implications
Mechanistic understanding is only one piece of the puzzle, and meaningful public health protections also depend on regulatory actions that reflect this emerging science. As knowledge of well-known and commonly employed PFAS compounds expands, new challenges emerge from newer PFAS variants, which pose complex challenges for health monitoring and regulatory development. The models developed after studying familiar compounds offer a good basis for the risk assessment of these new materials; however, they also highlight important knowledge gaps. Recent epidemiological studies have confirmed positive associations between PFOA, PFOS, PFNA, and PFHxS and liver injury or disease. Two independent high-exposure occupational cohorts (the C8 Health Project and an Italian fluorochemical worker cohort) both report elevated liver enzymes and increased liver cancer mortality linked to very high historical PFOA exposure [138,139]. Yet, there is little comprehensive work on newer PFAS compounds. This lack of information is concerning, given that molecular pathways elucidated in well-known PFAS suggest that even slight structural changes could lead to varying toxicity patterns while still being activated through similar pathways. Emerging PFAS compounds interacting with environmental and biological systems must respond to the same level of complexity. Interestingly, several molecular studies showed that these novel PFAS compounds exist in food supplies and show considerable liver toxicity [140,141]. Such liver toxicity in new compounds suggests that the liver injury mechanisms observed for established PFAS compounds may also apply to these newer variants, likely through similar nuclear receptor interactions as well as mitochondrial dysfunction pathways.
The regulatory challenges of these new PFAS compounds are significant. The risks associated with exposure cannot be ignored at the regulatory level [142]. Filling the knowledge gaps concerning these compounds will be of utmost importance, and science-based, evidence-based regulation will facilitate actions for improvement [143,144]. The mechanistic understanding developed for classic compounds offers a basis for deciding how to prioritize research toward new variants and appropriate approaches to risk assessment.
Emerging PFAS compounds show diverse structural architectures that can lead to unique toxicological characteristics. Some specific endocrine-disrupting PFAS compounds include C7-C13 perfluorocarboxylic acids, C4-C8 perfluorosulfonic acids, PFAS precursors, and GenX chemicals [140]. Based on the structure–activity relationships of earlier compounds, this may lead to distinct potencies and organ specificities with comparable basic mechanisms. New PFAS compounds pose serious health risks beyond liver damage, including effects on various organ systems in the body. Beyond hepatotoxicity, both legacy and emerging PFAS are increasingly associated with cardiovascular effects, including dyslipidemia, hypertension, and endothelial dysfunction [130]. PFOS, PFOA, and perfluorodecanoic acid (PFDA) have been shown to interfere with the regulation of thyroid hormones [141,142]. Epidemiologically, PFOA exposure is also associated with increased risks of kidney, prostate, and testicular cancers [142], whereas PFOS, PFOA, and possibly PFHxS and PFNA have been linked with significant immune-mediated toxicity [143,144]. PFOA exposure in women has been linked with reduced fertility, preeclampsia, and hypertension during pregnancy [144]. The potential developmental toxicity resulting from PFOA exposure on growth, cognitive function, and behavioral processes in childhood has also been implicated [144].
The health effects of classical PFAS pollutants provide a robust foundation for understanding what new variants can potentially do. These compounds disrupt nuclear receptors and cause mitochondrial problems or changes in metabolic pathways that lead to liver toxicity, which might also affect other organs. Notably, the endocrine-disrupting effects may also involve the same mechanisms as the metabolic changes seen in liver tissues [96,145,146].
Evaluating new PFAS agents is difficult, considering their structural differences and lack of toxicological information. However, what we have learned from studying well-established PFAS will continue to guide how we develop screening methods and direct future research. For instance, the nuclear receptor interactions, mitochondrial dysfunction, and metabolic disruptions that are relevant to PFAS-induced liver toxicity can provide a benchmark for evaluating potential toxic effects of these novel compounds [119,120,147]. Moreover, the structure–activity relationships occurring in common compounds demonstrate that chain length, functional groups, and protein-binding capacity of some of the new variants are likely to be important factors in their toxicity [121,122]. This mechanistic explanation leads to predictive models and enables the choice of acceptable testing systems for the evaluation of novel compounds [148]. When it comes to novel PFAS compounds, coupling this mechanistic information with exposure assessments is particularly important given insufficient epidemiological data [149]. The bioaccumulation and persistence properties associated with long-term exposure of established compounds are likely to be found in many new variants as well. This means that small exposures can add up to substantial body burdens over time.
10. Limitations and Future Directions
Although some advancements have been made to our understanding of PFAS hepatotoxicity, our ability to fully predict human health effects in terms of toxic substances and in the evaluation of possible emerging contaminants is limited by several significant limitations. Available in vitro models (e.g., 2D hepatocyte cultures and HepaRG cells) are limited based on the species-specific metabolic divergence and lack of tissue structure to characterize intact liver function [51,123]. Despite more advanced human-relevant receptor systems and the presence of 3D hepatocyte systems more approximate to chronic exposure conditions, these models do not yet reproduce the metabolic interactions, enterohepatic recirculation, and multiorgan crosstalk found in whole organisms. In animal models, interspecies variability in renal transporter expression, receptor activation thresholds, and metabolic enzyme profiles has a substantial role in dose–response interactions and toxicity [57,118,150], and similar limitations apply. However, the most drastic example of this species variability can be found in cholesterol metabolism, where PFAS exposure yields opposite effects in rodents compared to humans based upon PPARα expression patterns, receptor context, and dietary backgrounds [96,118,151]. One key unexplored area is that of PFAS mixtures, which better describe real-world exposure settings than single-compound studies [117,137]. The vast majority of experimental designs have investigated legacy compounds at high doses, but human subjects are exposed to dozens of PFAS at lower amounts in concurrent diets and/or drinking water and consumer products [22,23]. Mixture toxicity evaluations have been limited, especially for mixed mixtures of legacy and recently developed PFAS, which have remained ill defined in their interaction with additive, synergistic and antagonistic effects [117,123]. Moreover, the quick proliferation of chemical replacement has led to thousands of poorly characterized substitutes becoming available for commercial use, many of which are structurally similar to regulated products but lack basic toxicological characterization [152,153,154]. The issue is intensified by sparse analytical methods to analyze and quantify ultrashort-chain and polymeric PFAS, which might have different bioaccumulation and toxicity profiles [154].
Long-term epidemiological studies connecting PFAS exposure to hepatic and metabolic endpoints are required, especially with cohort studies that capture latency periods, sensitive life stages (prenatal and childhood) and cumulative exposures [87,124,127]. Biomonitoring strategy should no longer be limited to legacy compounds and instead include emerging PFAS and transformation products, and biomarker panels with the incorporation of a multi-omics approach will be crucial for subclinical manifestation [110,126]. Research priorities for the future should concentrate on a few aspects. First, the advent and validation of predictive quantitative structure–activity relationship (QSAR) models could lead to rapid hazard screening for emerging PFAS with respect to physicochemical properties and structural features and eliminate the need to perform more expensive toxicology testing on single compounds. Second, identification of such mechanistic biomarkers (metabolic patterns, mitochondrial parameters, and nuclear receptor activation profiles) would potentially help to detect PFAS-induced hepatotoxicity at an early stage and offer translatable endpoints for cross-modality model systems [110,126,131]. Thirdly, population sensitive studies such as pregnant women, infants, those with pre-existing metabolic disorders and occupationally exposed workers are crucial to characterize the risk variables and establish the limits for protective exposure [14,124,127]. Finally, incorporating multi-omics methodologies (transcriptomics, proteomics, metabolomics, and lipidomics) will allow systems-level information on PFAS toxicity and pinpoint convergent pathways that persist across chemical substitutions [110]. By addressing these knowledge gaps through integrated experimental and epidemiological approaches, the scientific community can provide the mechanistic foundation required for the evidence-based regulation and protection of public health.
11. Conclusions
The reviewed information describes the main hepatotoxicity mechanisms of PFAS by synthesizing toxicokinetic principles and molecular routes, as well as clinical data, to elucidate the way the long-term environmental pollutants are known to impair liver function. This is where nuclear receptor dysregulation (especially PPARα and CAR) becomes the driving components to toxic metabolic processes that are amplified by mitochondrial dysfunction via oxidative stress, β-oxidation dysfunction, and altered energy metabolism. Species-specific differences in receptor expression, metabolic enzyme profiles, and transporter activity greatly dictate the extent and type of toxicity responses, rendering direct extrapolation from animal models into human health risk assessment difficult. Importantly, the framework developed from legacy compound studies offers us a framework to predict toxic patterns in new PFAS, even though considerable research gaps persist. Although there is an accelerating awareness of the hazardous effects on health and the environment of PFAS, the extant regulatory approaches are fragmented and reactionary. Although the U.S. Environmental Protection Agency has made progress, namely with the PFAS Strategic Roadmap (2021–2024), an expansion of its goals regarding research, restriction and remediation, efforts have lagged behind the pace of scientific recognition of PFAS toxicity [155]. By not acting to change the current maximum contaminant levels (MCLs) for PFOA and PFOS, the agency is using a conservative response that ultimately misses the boat in dealing with the thousands of unregulated PFAS analogs currently used. Proposed rules to clarify supplier notification requirements for PFAS under the Toxics Release Inventory under the Toxic Substances Control Act (TSCA) essentially target manufacturers and not downstream users, thus leaving significant holes in data and accountability. Since there is no single federal standard for compliance, compliance obligations vary by state, which creates regulatory ambiguity for industries and enforcement challenges for policymakers. The mechanistic insights presented here highlight the need for class-based regulation that targets shared structural features as well as toxicological pathways, not thousands of PFAS alone. However, these substitution-based approaches have been ineffective, because new alternatives tend to possess the bioaccumulative nature and hepatotoxicity of legacy chemicals [152,153]. Robust policies must integrate mechanistic insight with epidemiological data to set exposure ceilings, expand environmental monitoring to evaluate new PFAS, and include sensitive populations in risk assessment frameworks. Although the EPA affirmed enforceable standards for PFOA and PFOS in May 2025, the simultaneous extension of compliance deadlines to 2031 and the rescission of regulatory determinations for other PFAS (such as GenX and PFNA) underscore the persistent tension between public health objectives and regulatory implementation. These shifts highlight the urgent need for a management strategy that integrates scientific research, transparent governance, and proactive policies supported by mechanistic toxicology studies to safeguard communities from ongoing PFAS exposure.
Author Contributions
Conceptualization, A.G. and N.A.-B.; A.G., M.K. and N.A.-B.; writing—review and editing, A.G. and N.A.-B.; supervision, N.A.-B. All authors have read and agreed to the published version of the manuscript.
Funding
Funding was provided by the National Institute of General Medical Sciences (NIGMS) P20 GM109005.
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
No new data were created or analyzed in this study. Data sharing is not applicable to this article.
Acknowledgments
During the preparation of this manuscript/study, Grammarly Version 1.2.91.1461 was used for copyediting and correction of typographical and grammatical errors. The authors have reviewed and edited the output and take full responsibility for the content of this publication.
Conflicts of Interest
The authors declare no conflicts of interest.
Abbreviations
The following abbreviations are used in this manuscript:
| 3D | Three-dimensional |
| ACOX1 | Acyl-CoA oxidase 1 |
| AFFF | Aqueous film-forming foam |
| AOP | Adverse outcome pathway |
| ASBT | Apical sodium-dependent bile acid transporter |
| ATSDR | Agency for Toxic Substances and Disease Registry |
| ATP | Adenosine triphosphate |
| ATP5B | ATP synthase subunit beta |
| BAF | Bioaccumulation factor |
| BCF | Bioconcentration factor |
| CAR | Constitutive androstane receptor |
| CYP | Cytochrome P450 |
| CYP2A6 | Cytochrome P450 2A6 |
| CYP2C9 | Cytochrome P450 2C9 |
| CYP2C19 | Cytochrome P450 2C19 |
| CYP7A1 | Cytochrome P450 7A1 (cholesterol 7-alpha hydroxylase) |
| DNA | Deoxyribonucleic acid |
| EFSA | European Food Safety Authority |
| EPA | United States Environmental Protection Agency |
| ER | Endoplasmic reticulum |
| FTOHs | Fluorotelomer alcohols |
| FXR | Farnesoid X receptor |
| GGT | Gamma-glutamyl transpeptidase |
| GSH | Glutathione |
| HBM4EU | Human Biomonitoring for Europe |
| HepaRG | Human hepatoma/hepatocyte cell line |
| HepG2 | Human hepatocellular carcinoma cell line |
| HFPO-DA | Hexafluoropropylene oxide dimer acid (GenX) |
| HFPO-TA | Hexafluoropropylene oxide trimer acid |
| HNF4α | Hepatocyte nuclear factor 4-alpha |
| IP3R2 | Inositol 1,4,5-trisphosphate receptor type 2 |
| KoNEHS | Korean National Environmental Health Survey |
| KOW | Octanol–water partition coefficient |
| L-02 | Human normal hepatocyte cell line (L-02) |
| LXR | Liver X receptor |
| MASLD | Metabolic-dysfunction-associated steatotic liver disease |
| MCL | Maximum contaminant level |
| MICU1 | Mitochondrial calcium uptake 1 |
| MIE | Molecular initiating event |
| NAFLD | Non-alcoholic fatty liver disease |
| NHANES | National Health and Nutrition Examination Survey |
| NLRP3 | NOD-like receptor protein 3 inflammasome |
| NTCP | Sodium taurocholate cotransporting polypeptide |
| OAT1 | Organic anion transporter 1 |
| OAT3 | Organic anion transporter 3 |
| OAT4 | Organic anion transporter 4 |
| OATP1B1 | Organic anion-transporting polypeptide 1B1 |
| OATP1B3 | Organic anion-transporting polypeptide 1B3 |
| OATP2B1 | Organic anion-transporting polypeptide 2B1 |
| OATPs | Organic anion-transporting polypeptides |
| PBW | Blood–water partitioning coefficient |
| PFAS | Per- and polyfluoroalkyl substances |
| PFBA | Perfluorobutanoic acid |
| PFBS | Perfluorobutanesulfonic acid |
| PFCAs | Perfluoroalkyl carboxylic acids |
| PFDA | Perfluorodecanoic acid |
| PFHpA | Perfluoroheptanoic acid |
| PFHxA | Perfluorohexanoic acid |
| PFHxS | Perfluorohexanesulfonic acid |
| PFNA | Perfluorononanoic acid |
| PFOA | Perfluorooctanoic acid |
| PFO4DA | Perfluoro-3,5,7,9-tetraoxadecanoic acid |
| PFO5DoDA | Perfluoro-3,5,7,9,11-pentaoxadodecanoic acid |
| PFOS | Perfluorooctanesulfonic acid |
| PFSAs | Perfluoroalkyl sulfonic acids |
| PPARα | Peroxisome proliferator-activated receptor alpha |
| PPARγ | Peroxisome proliferator-activated receptor gamma |
| PXR | Pregnane X receptor |
| QSAR | Quantitative structure–activity relationship |
| ROS | Reactive oxygen species |
| SIRT1 | Sirtuin 1 |
| SREBP | Sterol regulatory element-binding protein |
| TFA | Trifluoroacetate |
| TFR2 | Transferrin receptor 2 |
| TSCA | Toxic Substances Control Act |
| UCP2 | Uncoupling protein 2 |
| UPR | Unfolded protein response |
| URAT1 | Urate transporter 1 |
| VDAC1 | Voltage-dependent anion channel 1 |
References
- Gaines, L.G.T. Historical and current usage of per- and polyfluoroalkyl substances (PFAS): A literature review. Am. J. Ind. Med. 2023, 66, 353–378. [Google Scholar] [CrossRef] [Scilit]
- Schultes, L.; Vestergren, R.; Volkova, K.; Westberg, E.; Jacobson, T.; Benskin, J.P. Per- and polyfluoroalkyl substances and fluorine mass balance in cosmetic products from the Swedish market: Implications for environmental emissions and human exposure. Environ. Sci. Process. Impacts 2018, 20, 1680–1690. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Huang, K.; Li, Y.; Bu, D.; Fu, J.; Wang, M.; Zhou, W.; Gu, L.; Fu, Y.; Cong, Z.; Hu, B.; et al. Trophic Magnification of Short-Chain Per- and Polyfluoroalkyl Substances in a Terrestrial Food Chain from the Tibetan Plateau. Environ. Sci. Technol. Lett. 2022, 9, 147–152. [Google Scholar] [CrossRef] [Scilit]
- Munoz, G.; Mercier, L.; Duy, S.V.; Liu, J.; Sauvé, S.; Houde, M. Bioaccumulation and trophic magnification of emerging and legacy per- and polyfluoroalkyl substances (PFAS) in a St. Lawrence River food web. Environ. Pollut. 2022, 309, 119739. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Eun, H.; Yamazaki, E.; Taniyasu, S.; Miecznikowska, A.; Falandysz, J.; Yamashita, N. Evaluation of perfluoroalkyl substances in field-cultivated vegetables. Chemosphere 2020, 239, 124750. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, X.; Fang, M.; Bai, Z.; Zong, Y.; Zhao, S.; Zhan, J. Bioaccumulation, Biotransformation and Oxidative Stress of 6:2 Fluorotelomer Sulfonamidoalkyl Betaine (6:2 FTAB) in Earthworms (Eisenia fetida). Toxics 2025, 13, 337. [Google Scholar] [CrossRef] [Scilit]
- Macheka, L.R.; Olowoyo, J.O.; Mugivhisa, L.L.; Abafe, O.A. Determination and assessment of human dietary intake of per and polyfluoroalkyl substances in retail dairy milk and infant formula from South Africa. Sci. Total Environ. 2021, 755, 142697. [Google Scholar] [CrossRef] [Scilit]
- Xu, B.; Qiu, W.; Du, J.; Wan, Z.; Zhou, J.L.; Chen, H.; Liu, R.; Magnuson, J.T.; Zheng, C. Translocation, bioaccumulation, and distribution of perfluoroalkyl and polyfluoroalkyl substances (PFASs) in plants. iScience 2022, 25, 104061. [Google Scholar] [CrossRef] [Scilit]
- Scheurer, M.; Nödler, K. Ultrashort-chain perfluoroalkyl substance trifluoroacetate (TFA) in beer and tea—An unintended aqueous extraction. Food Chem. 2021, 351, 129304. [Google Scholar] [CrossRef] [Scilit]
- Monge Brenes, A.L.; Curtzwiler, G.; Dixon, P.; Harrata, K.; Talbert, J.; Vorst, K. PFOA and PFOS levels in microwave paper packaging between 2005 and 2018. Food Addit. Contam. Part B 2019, 12, 191–198. [Google Scholar] [CrossRef] [Scilit]
- Toptancı, İ.; Ketenoglu, O.; Kıralan, M. Assessment of the migration of perfluorinated compounds and primary aromatic amines from PTFE-coated non-stick cookware marketed in Turkey. Environ. Sci. Pollut. Res. 2022, 29, 38535–38549, Correction in Environ. Sci. Pollut. Res. 2022, 29, 38550. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lerch, M.; Nguyen, K.H.; Granby, K. Is the use of paper food contact materials treated with per- and polyfluorinated alkyl substances safe for high-temperature applications?—Migration study in real food and food simulants. Food Chem. 2022, 393, 133375. [Google Scholar] [CrossRef] [Scilit]
- Lerch, M.; Fengler, R.; Mbog, G.R.; Nguyen, K.H.; Granby, K. Food simulants and real food—What do we know about the migration of PFAS from paper based food contact materials? Food Packag. Shelf Life 2023, 35, 100992. [Google Scholar] [CrossRef] [Scilit]
- Augustsson, A.; Lennqvist, T.; Osbeck, C.M.G.; Tibblin, P.; Glynn, A.; Nguyen, M.A.; Westberg, E.; Vestergren, R. Consumption of freshwater fish: A variable but significant risk factor for PFOS exposure. Environ. Res. 2021, 192, 110284. [Google Scholar] [CrossRef] [Scilit]
- Onteeru, M.; Barnes, L.E.; O’Connell, K.; Bhimani, J.; Du, M.; Romano, M.E.; Kantor, E.D. Association between fish oil supplements use and serum per- and polyfluoroalkyl substances (PFAS): Results from the National Health and Nutrition Examination Survey. Environ. Res. 2022, 215, 114205. [Google Scholar] [CrossRef] [Scilit]
- Calafat, A.M.; Wong, L.Y.; Kuklenyik, Z.; Reidy, J.A.; Needham, L.L. Polyfluoroalkyl Chemicals in the U.S. Population: Data from the National Health and Nutrition Examination Survey (NHANES) 2003–2004 and Comparisons with NHANES 1999–2000. Environ. Health Perspect. 2007, 115, 1596–1602. [Google Scholar] [CrossRef] [Scilit]
- Botelho, J.C.; Kato, K.; Wong, L.Y.; Calafat, A.M. Per- and polyfluoroalkyl substances (PFAS) exposure in the U.S. population: NHANES 1999–March 2020. Environ. Res. 2025, 270, 120916. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Richterová, D.; Govarts, E.; Fábelová, L.; Rausová, K.; Rodriguez Martin, L.; Gilles, L.; Remy, S.; Colles, A.; Rambaud, L.; Riou, M.; et al. PFAS levels and determinants of variability in exposure in European teenagers—Results from the HBM4EU aligned studies (2014–2021). Int. J. Hyg. Environ. Health 2023, 247, 114057. [Google Scholar] [CrossRef] [Scilit]
- Bil, W.; Zeilmaker, M.; Fragki, S.; Lijzen, J.; Verbruggen, E.; Bokkers, B. Risk Assessment of Per- and Polyfluoroalkyl Substance Mixtures: A Relative Potency Factor Approach. Environ. Toxicol. Chem. 2020, 40, 859–870. [Google Scholar] [CrossRef] [Scilit]
- Hong, S.; Kim, O.J.; Jung, S.K.; Jeon, H.L.; Kim, S.; Kil, J. The Exposure Status of Environmental Chemicals in South Korea: The Korean National Environmental Health Survey 2018–2020. Toxics 2024, 12, 829. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lyu, Z.; Harada, K.H.; Kimura-Kuroda, J.; Tokuda, Y. Is Japan at low risk for PFAS immunotoxicity? Human biomonitoring study in contaminated areas in Japan. Environ. Health Prev. Med. 2024, 29, 37. [Google Scholar] [CrossRef] [Scilit]
- Christensen, K.Y.; Raymond, M.; Blackowicz, M.; Liu, Y.; Thompson, B.A.; Anderson, H.A.; Turyk, M. Perfluoroalkyl substances and fish consumption. Environ. Res. 2017, 154, 145–151. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fábelová, L.; Beneito, A.; Casas, M.; Colles, A.; Dalsager, L.; Den Hond, E.; Dereumeaux, C.; Ferguson, K.; Gilles, L.; Govarts, E.; et al. PFAS levels and exposure determinants in sensitive population groups. Chemosphere 2023, 313, 137530. [Google Scholar] [CrossRef] [Scilit]
- Kedikoglou, K.; Costopoulou, D.; Vassiliadou, I.; Leondiadis, L. Preliminary assessment of general population exposure to perfluoroalkyl substances through diet in Greece. Environ. Res. 2019, 177, 108617. [Google Scholar] [CrossRef] [Scilit]
- Abafe, O.A.; Macheka, L.R.; Abafe, O.T.; Chokwe, T.B. Concentrations and human exposure assessment of per and polyfluoroalkyl substances in farmed marine shellfish in South Africa. Chemosphere 2021, 281, 130985. [Google Scholar] [CrossRef] [Scilit]
- Lee, J.W.; Lee, H.K.; Lim, J.E.; Moon, H.B. Legacy and emerging per- and polyfluoroalkyl substances (PFASs) in the coastal environment of Korea: Occurrence, spatial distribution, and bioaccumulation potential. Chemosphere 2020, 251, 126633. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yu, J.; Nickerson, A.; Li, Y.; Fang, Y.; Strathmann, T.J. Fate of per- and polyfluoroalkyl substances (PFAS) during hydrothermal liquefaction of municipal wastewater treatment sludge. Environ. Sci. Water Res. Technol. 2020, 6, 1388–1399. [Google Scholar] [CrossRef] [Scilit]
- Bartolomé, M.; Gallego-Picó, A.; Cutanda, F.; Huetos, O.; Esteban, M.; Pérez-Gómez, B.; Castaño, A. Perfluorinated alkyl substances in Spanish adults: Geographical distribution and determinants of exposure. Sci. Total. Environ. 2017, 603–604, 352–360. [Google Scholar] [CrossRef] [Scilit]
- Colles, A.; Bruckers, L.; Den Hond, E.; Govarts, E.; Morrens, B.; Schettgen, T.; Buekers, J.; Coertjens, D.; Nawrot, T.; Loots, I.; et al. Perfluorinated substances in the Flemish population (Belgium): Levels and determinants of variability in exposure. Chemosphere 2020, 242, 125250. [Google Scholar] [CrossRef] [Scilit]
- LaKind, J.S.; Naiman, J.; Verner, M.A.; Lévêque, L.; Fenton, S. Per- and polyfluoroalkyl substances (PFAS) in breast milk and infant formula: A global issue. Environ. Res. 2023, 219, 115042. [Google Scholar] [CrossRef] [Scilit]
- Mamsen, L.S.; Björvang, R.D.; Mucs, D.; Vinnars, M.T.; Papadogiannakis, N.; Lindh, C.H.; Andersen, C.Y.; Damdimopoulou, P. Concentrations of perfluoroalkyl substances (PFASs) in human embryonic and fetal organs from first, second, and third trimester pregnancies. Environ. Int. 2019, 124, 482–492. [Google Scholar] [CrossRef] [Scilit]
- Spratlen, M.J.; Perera, F.P.; Lederman, S.A.; Rauh, V.A.; Robinson, M.; Kannan, K.; Trasande, L.; Herbstman, J. The association between prenatal exposure to perfluoroalkyl substances and childhood neurodevelopment. Environ. Pollut. 2020, 263, 114444. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, Y.; Fletcher, T.; Mucs, D.; Scott, K.; Lindh, C.H.; Tallving, P.; Jakobsson, K. Half-lives of PFOS, PFHxS and PFOA after end of exposure to contaminated drinking water. Occup. Environ. Med. 2018, 75, 46–51. [Google Scholar] [CrossRef] [Scilit]
- Brown, J.B.; Conder, J.M.; Arblaster, J.A.; Higgins, C.P. Assessing Human Health Risks from Per- and Polyfluoroalkyl Substance (PFAS)-Impacted Vegetable Consumption: A Tiered Modeling Approach. Environ. Sci. Technol. 2020, 54, 15202–15214. [Google Scholar] [CrossRef] [Scilit]
- Liu, J.J.; Cui, X.X.; Tan, Y.W.; Dong, P.X.; Ou, Y.Q.; Li, Q.Q.; Chu, C.; Wu, L.-Y.; Liang, L.-X.; Qin, S.-J.; et al. Per- and perfluoroalkyl substances alternatives, mixtures and liver function in adults: A community-based population study in China. Environ. Int. 2022, 163, 107179. [Google Scholar] [CrossRef] [Scilit]
- Jane LEspartero, L.; Yamada, M.; Ford, J.; Owens, G.; Prow, T.; Juhasz, A. Health-related toxicity of emerging per- and polyfluoroalkyl substances: Comparison to legacy PFOS and PFOA. Environ. Res. 2022, 212, 113431. [Google Scholar] [CrossRef] [Scilit]
- Jian, J.M.; Chen, D.; Han, F.J.; Guo, Y.; Zeng, L.; Lu, X.; Wang, F. A short review on human exposure to and tissue distribution of per- and polyfluoroalkyl substances (PFASs). Sci. Total Environ. 2018, 636, 1058–1069. [Google Scholar] [CrossRef] [Scilit]
- Fedorenko, M.; Alesio, J.; Fedorenko, A.; Slitt, A.; Bothun, G.D. Dominant entropic binding of perfluoroalkyl substances (PFASs) to albumin protein revealed by 19F NMR. Chemosphere 2021, 263, 128083. [Google Scholar] [CrossRef] [Scilit]
- Maso, L.; Trande, M.; Liberi, S.; Moro, G.; Daems, E.; Linciano, S.; Sobott, F.; Covaceuszach, S.; Cassetta, A.; Fasolato, S. Unveiling the binding mode of perfluorooctanoic acid to human serum albumin. Protein Sci. Publ. Protein Soc. 2021, 30, 830–841. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhao, L.; Teng, M.; Zhao, X.; Li, Y.; Sun, J.; Zhao, W.; Ruan, Y.; Leung, K.M.Y.; Wu, F. Insight into the binding model of per- and polyfluoroalkyl substances to proteins and membranes. Environ. Int. 2023, 175, 107951. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Rosato, I.; Bonato, T.; Fletcher, T.; Batzella, E.; Canova, C. Estimation of per- and polyfluoroalkyl substances (PFAS) half-lives in human studies: A systematic review and meta-analysis. Environ. Res. 2024, 242, 117743. [Google Scholar] [CrossRef] [Scilit]
- Forsthuber, M.; Kaiser, A.M.; Granitzer, S.; Hassl, I.; Hengstschläger, M.; Stangl, H.; Gundacker, C. Albumin is the major carrier protein for PFOS, PFOA, PFHxS, PFNA and PFDA in human plasma. Environ. Int. 2020, 137, 105324. [Google Scholar] [CrossRef] [Scilit]
- Poothong, S.; Papadopoulou, E.; Padilla-Sánchez, J.A.; Thomsen, C.; Haug, L.S. Multiple pathways of human exposure to poly- and perfluoroalkyl substances (PFASs): From external exposure to human blood. Environ. Int. 2020, 134, 105244. [Google Scholar] [CrossRef] [Scilit]
- Huang, M.C.; Dzierlenga, A.L.; Robinson, V.G.; Waidyanatha, S.; DeVito, M.J.; Eifrid, M.A.; Granville, C.A.; Gibbs, S.T.; Blystone, C.R. Toxicokinetics of perfluorobutane sulfonate (PFBS), perfluorohexane-1-sulphonic acid (PFHxS), and perfluorooctane sulfonic acid (PFOS) in male and female Hsd:Sprague Dawley SD rats after intravenous and gavage administration. Toxicol. Rep. 2019, 6, 645–655, Erratum in Toxicol. Rep. 2020, 8, 28–29. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gustafsson, Å.; Wang, B.; Gerde, P.; Bergman, Å.; Yeung, L.W.Y. Bioavailability of inhaled or ingested PFOA adsorbed to house dust. Environ. Sci. Pollut. Res. 2022, 29, 78698–78710. [Google Scholar] [CrossRef] [Scilit]
- Ragnarsdóttir, O.; Abdallah, M.A.E.; Harrad, S. Dermal uptake: An important pathway of human exposure to perfluoroalkyl substances? Environ. Pollut. 2022, 307, 119478. [Google Scholar] [CrossRef] [Scilit]
- Kowalczyk, J.; Ehlers, S.; Oberhausen, A.; Tischer, M.; Fürst, P.; Schafft, H.; Lahrssen-Wiederholt, M. Absorption, Distribution, and Milk Secretion of the Perfluoroalkyl Acids PFBS, PFHxS, PFOS, and PFOA by Dairy Cows Fed Naturally Contaminated Feed. J. Agric. Food Chem. 2013, 61, 2903–2912. [Google Scholar] [CrossRef] [Scilit]
- Zhao, W.; Zitzow, J.D.; Weaver, Y.; Ehresman, D.J.; Chang, S.C.; Butenhoff, J.L.; Hagenbuch, B. Organic Anion Transporting Polypeptides Contribute to the Disposition of Perfluoroalkyl Acids in Humans and Rats. Toxicol. Sci. 2017, 156, 84–95. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhao, W.; Zitzow, J.D.; Ehresman, D.J.; Chang, S.C.; Butenhoff, J.L.; Forster, J.; Hagenbuch, B. Na+/Taurocholate Cotransporting Polypeptide and Apical Sodium-Dependent Bile Acid Transporter Are Involved in the Disposition of Perfluoroalkyl Sulfonates in Humans and Rats. Toxicol. Sci. 2015, 146, 363–373. [Google Scholar] [CrossRef] [Scilit]
- Cao, H.; Zhou, Z.; Hu, Z.; Wei, C.; Li, J.; Wang, L.; Liu, G.; Zhang, J.; Wang, Y.; Wang, T.; et al. Effect of Enterohepatic Circulation on the Accumulation of Per- and Polyfluoroalkyl Substances: Evidence from Experimental and Computational Studies. Environ. Sci. Technol. 2022, 56, 3214–3224. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Louisse, J.; Fragki, S.; Rijkers, D.; Janssen, A.; Van Dijk, B.; Leenders, L.; Staats, M.; Bokkers, B.; Zeilmaker, M.; Piersma, A.; et al. Determination of in vitro hepatotoxic potencies of a series of perfluoroalkyl substances (PFASs) based on gene expression changes in HepaRG liver cells. Arch. Toxicol. 2023, 97, 1113–1131. [Google Scholar] [CrossRef] [Scilit]
- Li, J.; Wang, L.; Zhang, X.; Liu, P.; Deji, Z.; Xing, Y.; Zhou, Y.; Lin, X.; Huang, Z. Per- and polyfluoroalkyl substances exposure and its influence on the intestinal barrier: An overview on the advances. Sci. Total Environ. 2022, 852, 158362. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fischer, F.C.; Ludtke, S.; Thackray, C.; Pickard, H.M.; Haque, F.; Dassuncao, C.; Endo, S.; Schaider, L.; Sunderland, E.M. Binding of Per- and Polyfluoroalkyl Substances (PFAS) to Serum Proteins: Implications for Toxicokinetics in Humans. Environ. Sci. Technol. 2024, 58, 1055–1063. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Droge, S.T.J. Membrane–Water Partition Coefficients to Aid Risk Assessment of Perfluoroalkyl Anions and Alkyl Sulfates. Environ. Sci. Technol. 2019, 53, 760–770. [Google Scholar] [CrossRef] [Scilit]
- Koskela, A.; Koponen, J.; Lehenkari, P.; Viluksela, M.; Korkalainen, M.; Tuukkanen, J. Perfluoroalkyl substances in human bone: Concentrations in bones and effects on bone cell differentiation. Sci. Rep. 2017, 7, 6841. [Google Scholar] [CrossRef] [Scilit]
- Abraham, K.; El-Khatib, A.H.; Schwerdtle, T.; Monien, B.H. Perfluorobutanoic acid (PFBA): No high-level accumulation in human lung and kidney tissue. Int. J. Hyg. Environ. Health 2021, 237, 113830. [Google Scholar] [CrossRef] [Scilit]
- Nielsen, G.; Heiger-Bernays, W.J.; Schlezinger, J.J.; Webster, T.F. Predicting the effects of per- and polyfluoroalkyl substance mixtures on peroxisome proliferator-activated receptor alpha activity in vitro. Toxicology 2022, 465, 153024. [Google Scholar] [CrossRef] [Scilit]
- Baumert, B.O.; Fischer, F.C.; Nielsen, F.; Grandjean, P.; Bartell, S.; Stratakis, N.; Walker, D.I.; Valvi, D.; Kohli, R.; Inge, T.; et al. Paired Liver:Plasma PFAS Concentration Ratios from Adolescents in the Teen-LABS Study and Derivation of Empirical and Mass Balance Models to Predict and Explain Liver PFAS Accumulation. Environ. Sci. Technol. 2023, 57, 14817–14826. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, Y.; Lin, N.; Dai, C.; Xu, J.; Zhang, Y.; Xu, M.; Wang, F.; Li, Y.; Chen, D. Occurrence and distribution of per- and polyfluoroalkyl substances (PFASs) in human livers with liver cancer. Environ. Res. 2021, 202, 111775. [Google Scholar] [CrossRef] [Scilit]
- Cheng, W.; Ng, C.A. Predicting Relative Protein Affinity of Novel Per- and Polyfluoroalkyl Substances (PFASs) by An Efficient Molecular Dynamics Approach. Environ. Sci. Technol. 2018, 52, 7972–7980. [Google Scholar] [CrossRef] [Scilit]
- Burkhard, L.P. Evaluation of Published Bioconcentration Factor (BCF) and Bioaccumulation Factor (BAF) Data for Per- and Polyfluoroalkyl Substances Across Aquatic Species. Environ. Toxicol. Chem. 2021, 40, 1530–1543, Correction in Environ. Toxicol. Chem. 2021, 40, 2935–2940. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sims, J.L.; Cole, A.R.; Schmokel, C.; Kim, S.; Stroski, K.M.; Ehalt, R.; Simcik, M.F.; Brooks, B.W. Bioaccumulation and uptake kinetics of per- and polyfluoroalkyl substances in Pimephales promelas. Environ. Toxicol. Chem. 2025, 44, 1810–1823. [Google Scholar] [CrossRef] [Scilit]
- Qin, W.; Henneberger, L.; Huchthausen, J.; König, M.; Escher, B.I. Role of bioavailability and protein binding of four anionic perfluoroalkyl substances in cell-based bioassays for quantitative in vitro to in vivo extrapolations. Environ. Int. 2023, 173, 107857. [Google Scholar] [CrossRef] [Scilit]
- Chen, R.; Muensterman, D.; Field, J.; Ng, C. Deriving Membrane–Water and Protein–Water Partition Coefficients from In Vitro Experiments for Per- and Polyfluoroalkyl Substances (PFAS). Environ. Sci. Technol. 2025, 59, 82–91. [Google Scholar] [CrossRef] [Scilit]
- Pizzurro, D.M.; Seeley, M.; Kerper, L.E.; Beck, B.D. Interspecies differences in perfluoroalkyl substances (PFAS) toxicokinetics and application to health-based criteria. Regul. Toxicol. Pharmacol. 2019, 106, 239–250. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Glüge, J.; Scheringer, M.; Cousins, I.T.; DeWitt, J.C.; Goldenman, G.; Herzke, D.; Lohmann, R.; Ng, C.A.; Trier, X.; Wang, Z. An overview of the uses of per- and polyfluoroalkyl substances (PFAS). Environ. Sci. Process. Impacts 2020, 22, 2345–2373. [Google Scholar] [CrossRef] [Scilit]
- Mueller, R.; Yingling, V. History and Use of Per- and Polyfluoroalkyl Substances (PFAS); Interstate Technology & Regulatory Council: Washington, DC, USA, 2017. [Google Scholar]
- Kim, S.J.; Choi, E.J.; Choi, G.W.; Lee, Y.B.; Cho, H.Y. Exploring sex differences in human health risk assessment for PFNA and PFDA using a PBPK model. Arch. Toxicol. 2019, 93, 311–330. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dawson, D.E.; Lau, C.; Pradeep, P.; Sayre, R.R.; Judson, R.S.; Tornero-Velez, R.; Wambaugh, J.F. A Machine Learning Model to Estimate Toxicokinetic Half-Lives of Per- and Polyfluoro-Alkyl Substances (PFAS) in Multiple Species. Toxics 2023, 11, 98. [Google Scholar] [CrossRef] [Scilit]
- Lesmeister, L.; Lange, F.T.; Breuer, J.; Biegel-Engler, A.; Giese, E.; Scheurer, M. Extending the knowledge about PFAS bioaccumulation factors for agricultural plants—A review. Sci. Total Environ. 2021, 766, 142640. [Google Scholar] [CrossRef] [Scilit]
- Dzierlenga, M.W.; Crawford, L.; Longnecker, M.P. Birth weight and perfluorooctane sulfonic acid: A random-effects meta-regression analysis. Environ. Epidemiol. 2020, 4, e095. [Google Scholar] [CrossRef] [Scilit]
- Chang, C.J.; Young, A.S.; Keil, A.; Mullins, C.E.; Liang, D.; Zhao, S.; Jones, D.P.; Hu, X.; Walker, D.I.; White, A.J. Novel and legacy per- and polyfluoroalkyl substances in humans: Long-term temporal variability and metabolic perturbations. Environ. Int. 2025, 201, 109590. [Google Scholar] [CrossRef] [Scilit]
- Cohen Hubal, E.A. PFAS: Insights from Past Actions to Inform Today’s Decisions. J. Expo. Sci. Environ. Epidemiol. 2019, 29, 129–130. [Google Scholar] [CrossRef] [Scilit]
- Daramola, O.; Rand, A.A. Emerging investigator series: Human CYP2A6 catalyzes the oxidation of 6:2 fluorotelomer alcohol. Environ. Sci. Process. Impacts 2021, 23, 1688–1695. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- DeWitt, J.C.; Glüge, J.; Cousins, I.T.; Goldenman, G.; Herzke, D.; Lohmann, R.; Miller, M.; Ng, C.A.; Patton, S.; Trier, X.; et al. Zürich II Statement on Per- and Polyfluoroalkyl Substances (PFASs): Scientific and Regulatory Needs. Environ. Sci. Technol. Lett. 2024, 11, 786–797. [Google Scholar] [CrossRef] [Scilit]
- Agency for Toxic Substances and Disease Registry. 2021. Available online: https://www.atsdr.cdc.gov/reports/index.html (accessed on 15 October 2025).
- Ryu, S.; Yamaguchi, E.; Sadegh Modaresi, S.M.; Agudelo, J.; Costales, C.; West, M.A.; Fischer, F.; Slitt, A.L. Evaluation of 14 PFAS for permeability and organic anion transporter interactions: Implications for renal clearance in humans. Chemosphere 2024, 361, 142390. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Louisse, J.; Pedroni, L.; Van Den Heuvel, J.J.M.W.; Rijkers, D.; Leenders, L.; Noorlander, A.; Punt, A.; Russel, F.G.M.; Koenderink, J.B.; Dellafiora, L. In vitro and in silico characterization of the transport of selected perfluoroalkyl carboxylic acids and perfluoroalkyl sulfonic acids by human organic anion transporter 1 (OAT1), OAT2 and OAT3. Toxicology 2024, 509, 153961. [Google Scholar] [CrossRef] [Scilit]
- Ruggiero, M.J.; Miller, H.; Idowu, J.Y.; Zitzow, J.D.; Chang, S.C.; Hagenbuch, B. Perfluoroalkyl Carboxylic Acids Interact with the Human Bile Acid Transporter NTCP. Livers 2021, 1, 221–229. [Google Scholar] [CrossRef] [Scilit]
- Li, C.; Jiang, L.; Jin, Y.; Zhang, D.; Chen, J.; Qi, Y.; Fan, R.; Luo, J.; Xu, L.; Ma, W. Lipid metabolism disorders effects of 6:2 chlorinated polyfluorinated ether sulfonate through Hsa-miRNA-532–3p/Acyl-CoA oxidase 1(ACOX1) pathway. Ecotoxicol. Environ. Saf. 2021, 228, 113011. [Google Scholar] [CrossRef] [Scilit]
- Sheng, N.; Pan, Y.; Guo, Y.; Sun, Y.; Dai, J. Hepatotoxic Effects of Hexafluoropropylene Oxide Trimer Acid (HFPO-TA), A Novel Perfluorooctanoic Acid (PFOA) Alternative, on Mice. Environ. Sci. Technol. 2018, 52, 8005–8015. [Google Scholar] [CrossRef] [Scilit]
- Frangione, B.; Birk, S.; Benzouak, T.; Rodriguez-Villamizar, L.A.; Karim, F.; Dugandzic, R.; Villeneuve, P.J. Exposure to perfluoroalkyl and polyfluoroalkyl substances and pediatric obesity: A systematic review and meta-analysis. Int. J. Obes. 2024, 48, 131–146. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, Z.; Wang, G.; Braun, J.M.; Hong, X.; Choi, G.; O’Leary, S.P.; Yu, C.H.; Pearson, C.; Adams, W.G.; Fan, Z.; et al. Associations of early life per- and polyfluoroalkyl substances (PFAS) exposure with body mass index and risk of overweight or obesity at age 2–18 years: Mixture analysis in the prospective Boston Birth Cohort. Environ. Int. 2025, 195, 109206. [Google Scholar] [CrossRef] [Scilit]
- Sun, S.; Wang, J.; Yao, J.; Guo, H.; Dai, J. Transcriptome analysis of 3D primary mouse liver spheroids shows that long-term exposure to hexafluoropropylene oxide trimer acid disrupts hepatic bile acid metabolism. Sci. Total Environ. 2022, 812, 151509. [Google Scholar] [CrossRef] [Scilit]
- Roth, K.; Yang, Z.; Agarwal, M.; Liu, W.; Peng, Z.; Long, Z.; Birbeck, J.; Westrick, J.; Liu, W.; Petriello, M.C. Exposure to a mixture of legacy, alternative, and replacement per- and polyfluoroalkyl substances (PFAS) results in sex-dependent modulation of cholesterol metabolism and liver injury. Environ. Int. 2021, 157, 106843. [Google Scholar] [CrossRef] [Scilit]
- Schlezinger, J.J.; Hyötyläinen, T.; Sinioja, T.; Boston, C.; Puckett, H.; Oliver, J.; Heiger-Bernays, W.; Webster, T.F. Perfluorooctanoic acid induces liver and serum dyslipidemia in humanized PPARα mice fed an American diet. Toxicol. Appl. Pharmacol. 2021, 426, 115644. [Google Scholar] [CrossRef] [Scilit]
- Dunder, L.; Lind, P.M.; Salihovic, S.; Stubleski, J.; Kärrman, A.; Lind, L. Changes in plasma levels of per- and polyfluoroalkyl substances (PFAS) are associated with changes in plasma lipids—A longitudinal study over 10 years. Environ. Res. 2022, 211, 112903. [Google Scholar] [CrossRef] [Scilit]
- Reardon, A.J.F.; Rowan-Carroll, A.; Ferguson, S.S.; Leingartner, K.; Gagne, R.; Kuo, B.; Williams, A.; Lorusso, L.; Bourdon-Lacombe, J.A.; Carrier, R.; et al. Potency Ranking of Per- and Polyfluoroalkyl Substances Using High-Throughput Transcriptomic Analysis of Human Liver Spheroids. Toxicol. Sci. 2021, 184, 154–169. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wan, H.T.; Zhao, Y.G.; Wei, X.; Hui, K.Y.; Giesy, J.P.; Wong, C.K.C. PFOS-induced hepatic steatosis, the mechanistic actions on β-oxidation and lipid transport. Biochim. Biophys. Acta BBA-Gen. Subj. 2012, 1820, 1092–1101. [Google Scholar] [CrossRef] [Scilit]
- Zheng, P.; Liu, Y.; An, Q.; Yang, X.; Yin, S.; Ma, L.Q.; Liu, W. Prenatal and postnatal exposure to emerging and legacy per-/polyfluoroalkyl substances: Levels and transfer in maternal serum, cord serum, and breast milk. Sci. Total Environ. 2022, 812, 152446. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zheng, F.; Sheng, N.; Zhang, H.; Yan, S.; Zhang, J.; Wang, J. Perfluorooctanoic acid exposure disturbs glucose metabolism in mouse liver. Toxicol. Appl. Pharmacol. 2017, 335, 41–48. [Google Scholar] [CrossRef] [Scilit]
- Chen, J.; Li, H.; Yao, J.; Guo, H.; Zhang, H.; Guo, Y.; Sheng, N.; Wang, J.; Dai, J. Chronic exposure to PFO4DA and PFO5DoDA, two perfluoroalkyl ether carboxylic acids (PFECAs), suppresses hepatic stress signals and disturbs glucose and lipid metabolism in male mice. J. Hazard. Mater. 2021, 411, 124963. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Marques, E.; Pfohl, M.; Wei, W.; Tarantola, G.; Ford, L.; Amaeze, O.; Alesio, J.; Ryu, S.; Jia, X.; Zhu, H.; et al. Replacement per- and polyfluoroalkyl substances (PFAS) are potent modulators of lipogenic and drug metabolizing gene expression signatures in primary human hepatocytes. Toxicol. Appl. Pharmacol. 2022, 442, 115991. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Qi, W.; Clark, J.M.; Timme-Laragy, A.R.; Park, Y. Perfluorobutanesulfonic acid (PFBS) induces fat accumulation in HepG2 human hepatoma. Toxicol. Environ. Chem. 2020, 102, 585–606. [Google Scholar] [CrossRef] [Scilit]
- Behr, A.; Kwiatkowski, A.; Stahlman, M.; Schmidt, F.F.; Luckert, C.; Braeuning, A.; Buhrke, T. Correction to: Impairment of bile acid metabolism by perfluorooctanoic acid (PFOA) and perfluorooctanesulfonic acid (PFOS) in human HepaRG hepatoma cells. Arch. Toxicol. 2021, 95, 2891. [Google Scholar] [CrossRef] [Scilit]
- Attema, B.; Janssen, A.W.F.; Rijkers, D.; Van Schothorst, E.M.; Hooiveld, G.J.E.J.; Kersten, S. Exposure to low-dose perfluorooctanoic acid promotes hepatic steatosis and disrupts the hepatic transcriptome in mice. Mol. Metab. 2022, 66, 101602. [Google Scholar] [CrossRef] [Scilit]
- Abe, T.; Takahashi, M.; Kano, M.; Amaike, Y.; Ishii, C.; Maeda, K.; Kudoh, Y.; Morishita, T.; Hosaka, T.; Sasaki, T.; et al. Activation of nuclear receptor CAR by an environmental pollutant perfluorooctanoic acid. Arch. Toxicol. 2017, 91, 2365–2374. [Google Scholar] [CrossRef] [Scilit]
- Li, R.; Zhang, Z.; Xuan, Y.; Wang, Y.; Zhong, Y.; Zhang, L.; Zhang, J.; Chen, Q.; Yu, S.; Yuan, J. HNF4A as a potential target of PFOA and PFOS leading to hepatic steatosis: Integrated molecular docking, molecular dynamic and transcriptomic analyses. Chem. Biol. Interact. 2024, 390, 110867. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Costello, E.; Rock, S.; Stratakis, N.; Eckel, S.P.; Walker, D.I.; Valvi, D.; Cserbik, D.; Jenkins, T.; Xanthakos, S.A.; Kohli, R.; et al. Exposure to per- and Polyfluoroalkyl Substances and Markers of Liver Injury: A Systematic Review and Meta-Analysis. Environ. Health Perspect. 2022, 130, 46001. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Louisse, J.; Rijkers, D.; Stoopen, G.; Janssen, A.; Staats, M.; Hoogenboom, R.; Kersten, S.; Peijnenburg, A. Perfluorooctanoic acid (PFOA), perfluorooctane sulfonic acid (PFOS), and perfluorononanoic acid (PFNA) increase triglyceride levels and decrease cholesterogenic gene expression in human HepaRG liver cells. Arch. Toxicol. 2020, 94, 3137–3155. [Google Scholar] [CrossRef] [Scilit]
- Fragki, S.; Dirven, H.; Fletcher, T.; Grasl-Kraupp, B.; Bjerve Gützkow, K.; Hoogenboom, R.; Kersten, S.; Lindeman, B.; Louisse, J.; Peijnenburg, A.; et al. Systemic PFOS and PFOA exposure and disturbed lipid homeostasis in humans: What do we know and what not? Crit. Rev. Toxicol. 2021, 51, 141–164. [Google Scholar] [CrossRef] [Scilit]
- Yang, W.; Ling, X.; He, S.; Cui, H.; Yang, Z.; An, H.; Wang, L.; Zou, P.; Chen, Q.; Liu, J.; et al. PPARα/ACOX1 as a novel target for hepatic lipid metabolism disorders induced by per- and polyfluoroalkyl substances: An integrated approach. Environ. Int. 2023, 178, 108138. [Google Scholar] [CrossRef] [Scilit]
- Evans, N.; Conley, J.M.; Cardon, M.; Hartig, P.; Medlock-Kakaley, E.; Gray, L.E. In vitro activity of a panel of per- and polyfluoroalkyl substances (PFAS), fatty acids, and pharmaceuticals in peroxisome proliferator-activated receptor (PPAR) alpha, PPAR gamma, and estrogen receptor assays. Toxicol. Appl. Pharmacol. 2022, 449, 116136. [Google Scholar] [CrossRef] [Scilit]
- Maeda, K.; Hirano, M.; Hayashi, T.; Iida, M.; Kurata, H.; Ishibashi, H. Elucidating Key Characteristics of PFAS Binding to Human Peroxisome Proliferator-Activated Receptor Alpha: An Explainable Machine Learning Approach. Environ. Sci. Technol. 2024, 58, 488–497. [Google Scholar] [CrossRef] [Scilit]
- Jin, R.; McConnell, R.; Catherine, C.; Xu, S.; Walker, D.I.; Stratakis, N.; Jones, D.P.; Miller, G.W.; Peng, C.; Conti, D.V.; et al. Perfluoroalkyl substances and severity of nonalcoholic fatty liver in Children: An untargeted metabolomics approach. Environ. Int. 2020, 134, 105220. [Google Scholar] [CrossRef] [Scilit]
- Sen, P.; Qadri, S.; Luukkonen, P.K.; Ragnarsdottir, O.; McGlinchey, A.; Jäntti, S.; Juuti, A.; Arola, J.; Schlezinger, J.J.; Webster, T.F.; et al. Exposure to environmental contaminants is associated with altered hepatic lipid metabolism in non-alcoholic fatty liver disease. J. Hepatol. 2022, 76, 283–293. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cao, L.; Guo, Y.; Chen, Y.; Hong, J.; Wu, J.; Hangbiao, J. Per-/polyfluoroalkyl substance concentrations in human serum and their associations with liver cancer. Chemosphere 2022, 296, 134083. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, Z.; Yang, T.; Walker, D.I.; Thomas, D.C.; Qiu, C.; Chatzi, L.; Alderete, T.L.; Kim, J.S.; Conti, D.V.; Breton, C.V.; et al. Dysregulated lipid and fatty acid metabolism link perfluoroalkyl substances exposure and impaired glucose metabolism in young adults. Environ. Int. 2020, 145, 106091. [Google Scholar] [CrossRef] [Scilit]
- Cheng, W.; Li, M.; Zhang, L.; Zhou, C.; Zhang, X.; Zhu, C.; Tan, L.; Lin, H.; Zhang, W.; Zhang, W. Close association of PFASs exposure with hepatic fibrosis than steatosis: Evidences from NHANES 2017–2018. Ann. Med. 2023, 55, 2216943. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Guo, P.; Furnary, T.; Vasiliou, V.; Yan, Q.; Nyhan, K.; Jones, D.P.; Johnson, C.H.; Liew, Z. Non-targeted metabolomics and associations with per- and polyfluoroalkyl substances (PFAS) exposure in humans: A scoping review. Environ. Int. 2022, 162, 107159. [Google Scholar] [CrossRef] [Scilit]
- Ojo, A.F.; Peng, C.; Ng, J.C. Genotoxicity assessment of per- and polyfluoroalkyl substances mixtures in human liver cells (HepG2). Toxicology 2022, 482, 153359. [Google Scholar] [CrossRef] [Scilit]
- Wen, Y.; Mirji, N.; Irudayaraj, J. Epigenetic toxicity of PFOA and GenX in HepG2 cells and their role in lipid metabolism. Toxicol. In Vitro 2020, 65, 104797. [Google Scholar] [CrossRef] [Scilit]
- Yoo, H.J.; Pyo, M.C.; Park, Y.; Kim, B.Y.; Lee, K.W. Hexafluoropropylene oxide dimer acid (GenX) exposure induces apoptosis in HepG2 cells. Heliyon 2021, 7, e08272. [Google Scholar] [CrossRef] [Scilit]
- Ojo, A.F.; Peng, C.; Ng, J.C. Combined effects and toxicological interactions of perfluoroalkyl and polyfluoroalkyl substances mixtures in human liver cells (HepG2). Environ. Pollut. 2020, 263, 114182. [Google Scholar] [CrossRef] [Scilit]
- Wang, X.; Lv, Y.; Qiang, X.; Liang, S.; Li, R.; Zhan, J.; Liu, J. Perfluorooctanoic acid (PFOA) and its alternative perfluorobutanoic acid (PFBA) alter hepatic bile acid profiles via different pathways. Sci. Total Environ. 2024, 950, 175312. [Google Scholar] [CrossRef] [Scilit]
- Zhang, R.; Lu, W.; Yao, Y.; Tu, L.; Yu, T.; Luan, T.; Chen, B. Metabolomics analysis of the 3D L-02 cell cultures revealing the key role of metabolism of amino acids in ameliorating hepatotoxicity of perfluorooctanoic acid. Sci. Total Environ. 2022, 806, 150438. [Google Scholar] [CrossRef] [Scilit]
- Khan, E.A.; Grønnestad, R.; Krøkje, Å.; Bartosov, Z.; Johanson, S.M.; Müller, M.H.B.; Arukwe, A. Alteration of hepato-lipidomic homeostasis in A/J mice fed an environmentally relevant PFAS mixture. Environ. Int. 2023, 173, 107838. [Google Scholar] [CrossRef] [Scilit]
- Nielsen, G.; Gondim, D.D.; Cave, M.C.; Heiger-Bernays, W.J.; Webster, T.F.; Schlezinger, J.J. Perfluorooctanoic acid increases serum cholesterol in a PPARα-dependent manner in female mice. Arch. Toxicol. 2025, 99, 2087–2105. [Google Scholar] [CrossRef] [Scilit]
- Kashobwe, L.; Sadrabadi, F.; Brunken, L.; Coelho, A.C.M.F.; Sandanger, T.M.; Braeuning, A.; Buhrke, T.; Öberg, M.; Hamers, T.; Leonards, P.i.m.E.G. Legacy and alternative per- and polyfluoroalkyl substances (PFAS) alter the lipid profile of HepaRG cells. Toxicology 2024, 506, 153862. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ford, L.C.; Lin, H.C.; Tsai, H.H.D.; Zhou, Y.H.; Wright, F.A.; Sedykh, A.; Shah, R.R.; Chiu, W.A.; Rusyn, I. Hazard and risk characterization of 56 structurally diverse PFAS using a targeted battery of broad coverage assays using six human cell types. Toxicology 2024, 503, 153763. [Google Scholar] [CrossRef] [Scilit]
- Leuthner, T.C.; Zhang, S.; Kohrn, B.F.; Stapleton, H.M.; Baugh, L.R. Structure-specific variation in per- and polyfluoroalkyl substances toxicity among genetically diverse Caenorhabditis elegans strains. Toxicol. Sci. 2025, 205, 205–219. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Amstutz, V.H.; Mircheva, A.; Cengo, A.; Dubois, L.J.; Sijm, D.T.H.M.; Vrolijk, M.F. A subcellular study on reactive oxygen species generation by PFAS in HepG2 cells. Sci. Rep. 2025, 15, 21914. [Google Scholar] [CrossRef] [Scilit]
- Sadrabadi, F.; Alarcan, J.; Sprenger, H.; Braeuning, A.; Buhrke, T. Impact of perfluoroalkyl substances (PFAS) and PFAS mixtures on lipid metabolism in differentiated HepaRG cells as a model for human hepatocytes. Arch. Toxicol. 2024, 98, 507–524. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Stratakis, N.; Conti, D.V.; Jin, R.; Margetaki, K.; Valvi, D.; Siskos, A.P.; Maitre, L.; Garcia, E.; Varo, N.; Zhao, Y.; et al. Prenatal Exposure to Perfluoroalkyl Substances Associated With Increased Susceptibility to Liver Injury in Children. Hepatology 2020, 72, 1758–1770. [Google Scholar] [CrossRef] [Scilit]
- Sun, X.; Yu, Q.; Kang, B.; Zhao, X.; Li, H.; Liu, H.; Wang, P.; Cong, M.; Liu, T. Diethyldithiocarbamate inhibits the activation of hepatic stellate cells via PPARα/FABP1 in mice with non-alcoholic steatohepatitis. Biochem. Biophys. Res. Commun. 2023, 641, 192–199. [Google Scholar] [CrossRef] [Scilit]
- Lu, Y.; Gao, K.; Li, X.; Tang, Z.; Xiang, L.; Zhao, H.; Fu, J.; Wang, L.; Zhu, N.; Cai, Z.; et al. Mass Spectrometry-Based Metabolomics Reveals Occupational Exposure to Per- and Polyfluoroalkyl Substances Relates to Oxidative Stress, Fatty Acid β-Oxidation Disorder, and Kidney Injury in a Manufactory in China. Environ. Sci. Technol. 2019, 53, 9800–9809. [Google Scholar] [CrossRef] [Scilit]
- Li, S.; Oliva, P.; Zhang, L.; Goodrich, J.A.; McConnell, R.; Conti, D.V.; Chatzi, L.; Aung, M. Associations between per-and polyfluoroalkyl substances (PFAS) and county-level cancer incidence between 2016 and 2021 and incident cancer burden attributable to PFAS in drinking water in the United States. J. Expo. Sci. Environ. Epidemiol. 2025, 35, 425–436. [Google Scholar] [CrossRef] [Scilit]
- Wang, J.; Wang, J.; Qiu, T.; Wu, J.; Sun, X.; Jiang, L.; Liu, X.; Yang, G.; Cao, J.; Yao, X. Mitochondrial iron overload mediated by cooperative transfer of plasma membrane ATP5B and TFR2 to mitochondria triggers hepatic insulin resistance under PFOS exposure. Ecotoxicol. Environ. Saf. 2023, 253, 114662. [Google Scholar] [CrossRef] [Scilit]
- Dong, Z.; Wang, J.; Qiu, T.; Wu, J.; An, Y.; Shi, X.; Sun, X.; Jiang, L.; Liu, X.; Yang, G.; et al. Perfluorooctane sulfonate induces mitochondrial calcium overload and early hepatic insulin resistance via autophagy/detyrosinated alpha-tubulin-regulated IP3R2-VDAC1-MICU1 interaction. Sci. Total Environ. 2022, 825, 153933. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wen, Z.J.; Wei, Y.J.; Zhang, Y.F.; Zhang, Y.F. A review of cardiovascular effects and underlying mechanisms of legacy and emerging per- and polyfluoroalkyl substances (PFAS). Arch. Toxicol. 2023, 97, 1195–1245. [Google Scholar] [CrossRef] [Scilit]
- Schillemans, T.; Shi, L.; Donat-Vargas, C.; Hanhineva, K.; Tornevi, A.; Johansson, I.; Koponen, J.; Kiviranta, H.; Rolandsson, O.; Bergdahl, I.A.; et al. Plasma metabolites associated with exposure to perfluoroalkyl substances and risk of type 2 diabetes—A nested case-control study. Environ. Int. 2021, 146, 106180. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gong, X.; Yang, C.; Hong, Y.; Chung, A.C.K.; Cai, Z. PFOA and PFOS promote diabetic renal injury in vitro by impairing the metabolisms of amino acids and purines. Sci. Total Environ. 2019, 676, 72–86. [Google Scholar] [CrossRef] [Scilit]
- Duan, X.; Sun, W.; Sun, H.; Zhang, L. Perfluorooctane sulfonate continual exposure impairs glucose-stimulated insulin secretion via SIRT1-induced upregulation of UCP2 expression. Environ. Pollut. 2021, 278, 116840. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wei, K.N.; Wang, X.J.; Zeng, Z.C.; Gu, R.T.; Deng, S.Z.; Jiang, J.; Xu, C.-L.; Li, W.; Wang, H.-L. Perfluorooctane sulfonate affects mouse oocyte maturation in vitro by promoting oxidative stress and apoptosis induced bymitochondrial dysfunction. Ecotoxicol. Environ. Saf. 2021, 225, 112807. [Google Scholar] [CrossRef] [Scilit]
- Jiao, X.; Liu, N.; Xu, Y.; Qiao, H. Perfluorononanoic acid impedes mouse oocyte maturation by inducing mitochondrial dysfunction and oxidative stress. Reprod. Toxicol. 2021, 104, 58–67. [Google Scholar] [CrossRef] [Scilit]
- Zhao, Y.; Zhao, H.; Xu, H.; An, P.; Ma, B.; Lu, H.; Zhou, Q.; Li, X.; Xiong, Y. Perfluorooctane sulfonate exposure induces preeclampsia-like syndromes by damaging trophoblast mitochondria in pregnant mice. Ecotoxicol. Environ. Saf. 2022, 247, 114256. [Google Scholar] [CrossRef] [Scilit]
- Liu, Y.; Liu, S.; Huang, J.; Liu, Y.; Wang, Q.; Chen, J.; Sun, L.; Tu, W. Mitochondrial dysfunction in metabolic disorders induced by per- and polyfluoroalkyl substance mixtures in zebrafish larvae. Environ. Int. 2023, 176, 107977. [Google Scholar] [CrossRef] [Scilit]
- Andres, K.L.; Olsen, G.W.; Krisko, R.M.; Nunnally, M.C.; Boeding, R.R.; Leniek, K.L.; Taiwo, O.A. An investigation of 3M Cordova, IL production worker’s per- and polyfluoroalkyl substances biomonitoring results and mortality experience. Int. J. Hyg. Environ. Health 2024, 256, 114321. [Google Scholar] [CrossRef] [Scilit]
- Girardi, P.; Merler, E. A mortality study on male subjects exposed to polyfluoroalkyl acids with high internal dose of perfluorooctanoic acid. Environ. Res. 2019, 179, 108743. [Google Scholar] [CrossRef] [Scilit]
- Panieri, E.; Buha-Djordjević, A.; Saso, L. Endocrine disruption by PFAS: A major concern associated with legacy and replacement substances. Arh. Farm. 2021, 71, 429–454. [Google Scholar] [CrossRef] [Scilit]
- Lau, C. Perfluorinated Compounds. In Molecular, Clinical and Environmental Toxicology; (Experientia Supplementum); Luch, A., Ed.; Springer: Basel, Switzerland, 2012; pp. 47–86. [Google Scholar] [CrossRef] [Scilit]
- Steenland, K.; Winquist, A. PFAS and cancer, a scoping review of the epidemiologic evidence. Environ. Res. 2021, 194, 110690. [Google Scholar] [CrossRef] [Scilit]
- Von Holst, H.; Nayak, P.; Dembek, Z.; Buehler, S.; Echeverria, D.; Fallacara, D.; John, L. Perfluoroalkyl substances exposure and immunity, allergic response, infection, and asthma in children: Review of epidemiologic studies. Heliyon 2021, 7, e08160. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Anderko, L.; Pennea, E. Exposures to per-and polyfluoroalkyl substances (PFAS): Potential risks to reproductive and children’s health. Curr. Probl. Pediatr. Adolesc. Health Care 2020, 50, 100760. [Google Scholar] [CrossRef] [Scilit]
- Zheng, H.; Yin, Z.; Luo, X.; Zhou, Y.; Zhang, F.; Guo, Z. Association of per- and polyfluoroalkyl substance exposure with metabolic syndrome and its components in adults and adolescents. Environ. Sci. Pollut. Res. 2023, 30, 112943–112958. [Google Scholar] [CrossRef] [Scilit]
- Lewis, N.; Abdulkadir, A.; Kandel, S.; Rosby, R.; Hossain, E. Per- and Polyfluoroalkyl Substances (PFAS) as Emerging Obesogens: Mechanisms, Epidemiological Evidence, and Regulatory Challenges. Physiologia 2024, 4, 517–567. [Google Scholar] [CrossRef] [Scilit]
- Mišľanová, C.; Valachovičová, M. Health Impacts of Per- and Polyfluoroalkyl Substances (PFASs): A Comprehensive Review. Life 2025, 15, 573. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yin, Z.; Zhang, M.; Liu, R.; Cai, Y. Explainable machine learning models enhance prediction of PFAS bioactivity using quantitative molecular surface analysis-derived representation. Water Res. 2025, 280, 123500. [Google Scholar] [CrossRef] [Scilit]
- Mikkonen, A.T.; Martin, J.; Upton, R.N.; Moenning, J.L.; Numata, J.; Taylor, M.P.; Roberts, M.S.; Mackenzie, L. Dynamic exposure and body burden models for per- and polyfluoroalkyl substances (PFAS) enable management of food safety risks in cattle. Environ. Int. 2023, 180, 108218. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kersten, S.; Stienstra, R. The role and regulation of the peroxisome proliferator activated receptor alpha in human liver. Biochimie 2017, 136, 75–84. [Google Scholar] [CrossRef] [Scilit]
- Schlezinger, J.J.; Puckett, H.; Oliver, J.; Nielsen, G.; Heiger-Bernays, W.; Webster, T.F. Perfluorooctanoic acid activates multiple nuclear receptor pathways and skews expression of genes regulating cholesterol homeostasis in liver of humanized PPARα mice fed an American diet. Toxicol. Appl. Pharmacol. 2020, 405, 115204. [Google Scholar] [CrossRef] [Scilit]
- Itumoh, E.J.; Data, S.; Chen, J.L.Y.; Kah, M.; Padhye, L.P.; Leitao, E.M. Addressing the persistence of per- and poly-fluoroalkyl substances (PFAS): Current challenges and potential solutions. RSC Sustain. 2024, 2, 3183–3201. [Google Scholar] [CrossRef] [Scilit]
- Dosunmu, O.; Whiting, R.; Matharu, A.; Watson, N.; Sweetman, A.J. The unintentional role of chemical regulation in regrettable substitution: The case of PFAS. Environ. Sci. Policy 2025, 174, 104275. [Google Scholar] [CrossRef] [Scilit]
- Maerten, A.; Sanz-Serrano, J.; Devisscher, L.; Vinken, M. Tiny molecules, big concerns: Ultrashort-chain PFAS on the regulatory radar. Arch. Toxicol. 2025, 99, 3449–3451. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- PFAS Strategic Roadmap: EPA’s Commitments to Action 2021–2024. Available online: https://www.epa.gov/pfas/pfas-strategic-roadmap-epas-commitments-action-2021-2024 (accessed on 15 October 2025).
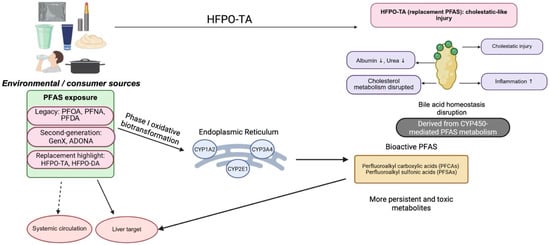
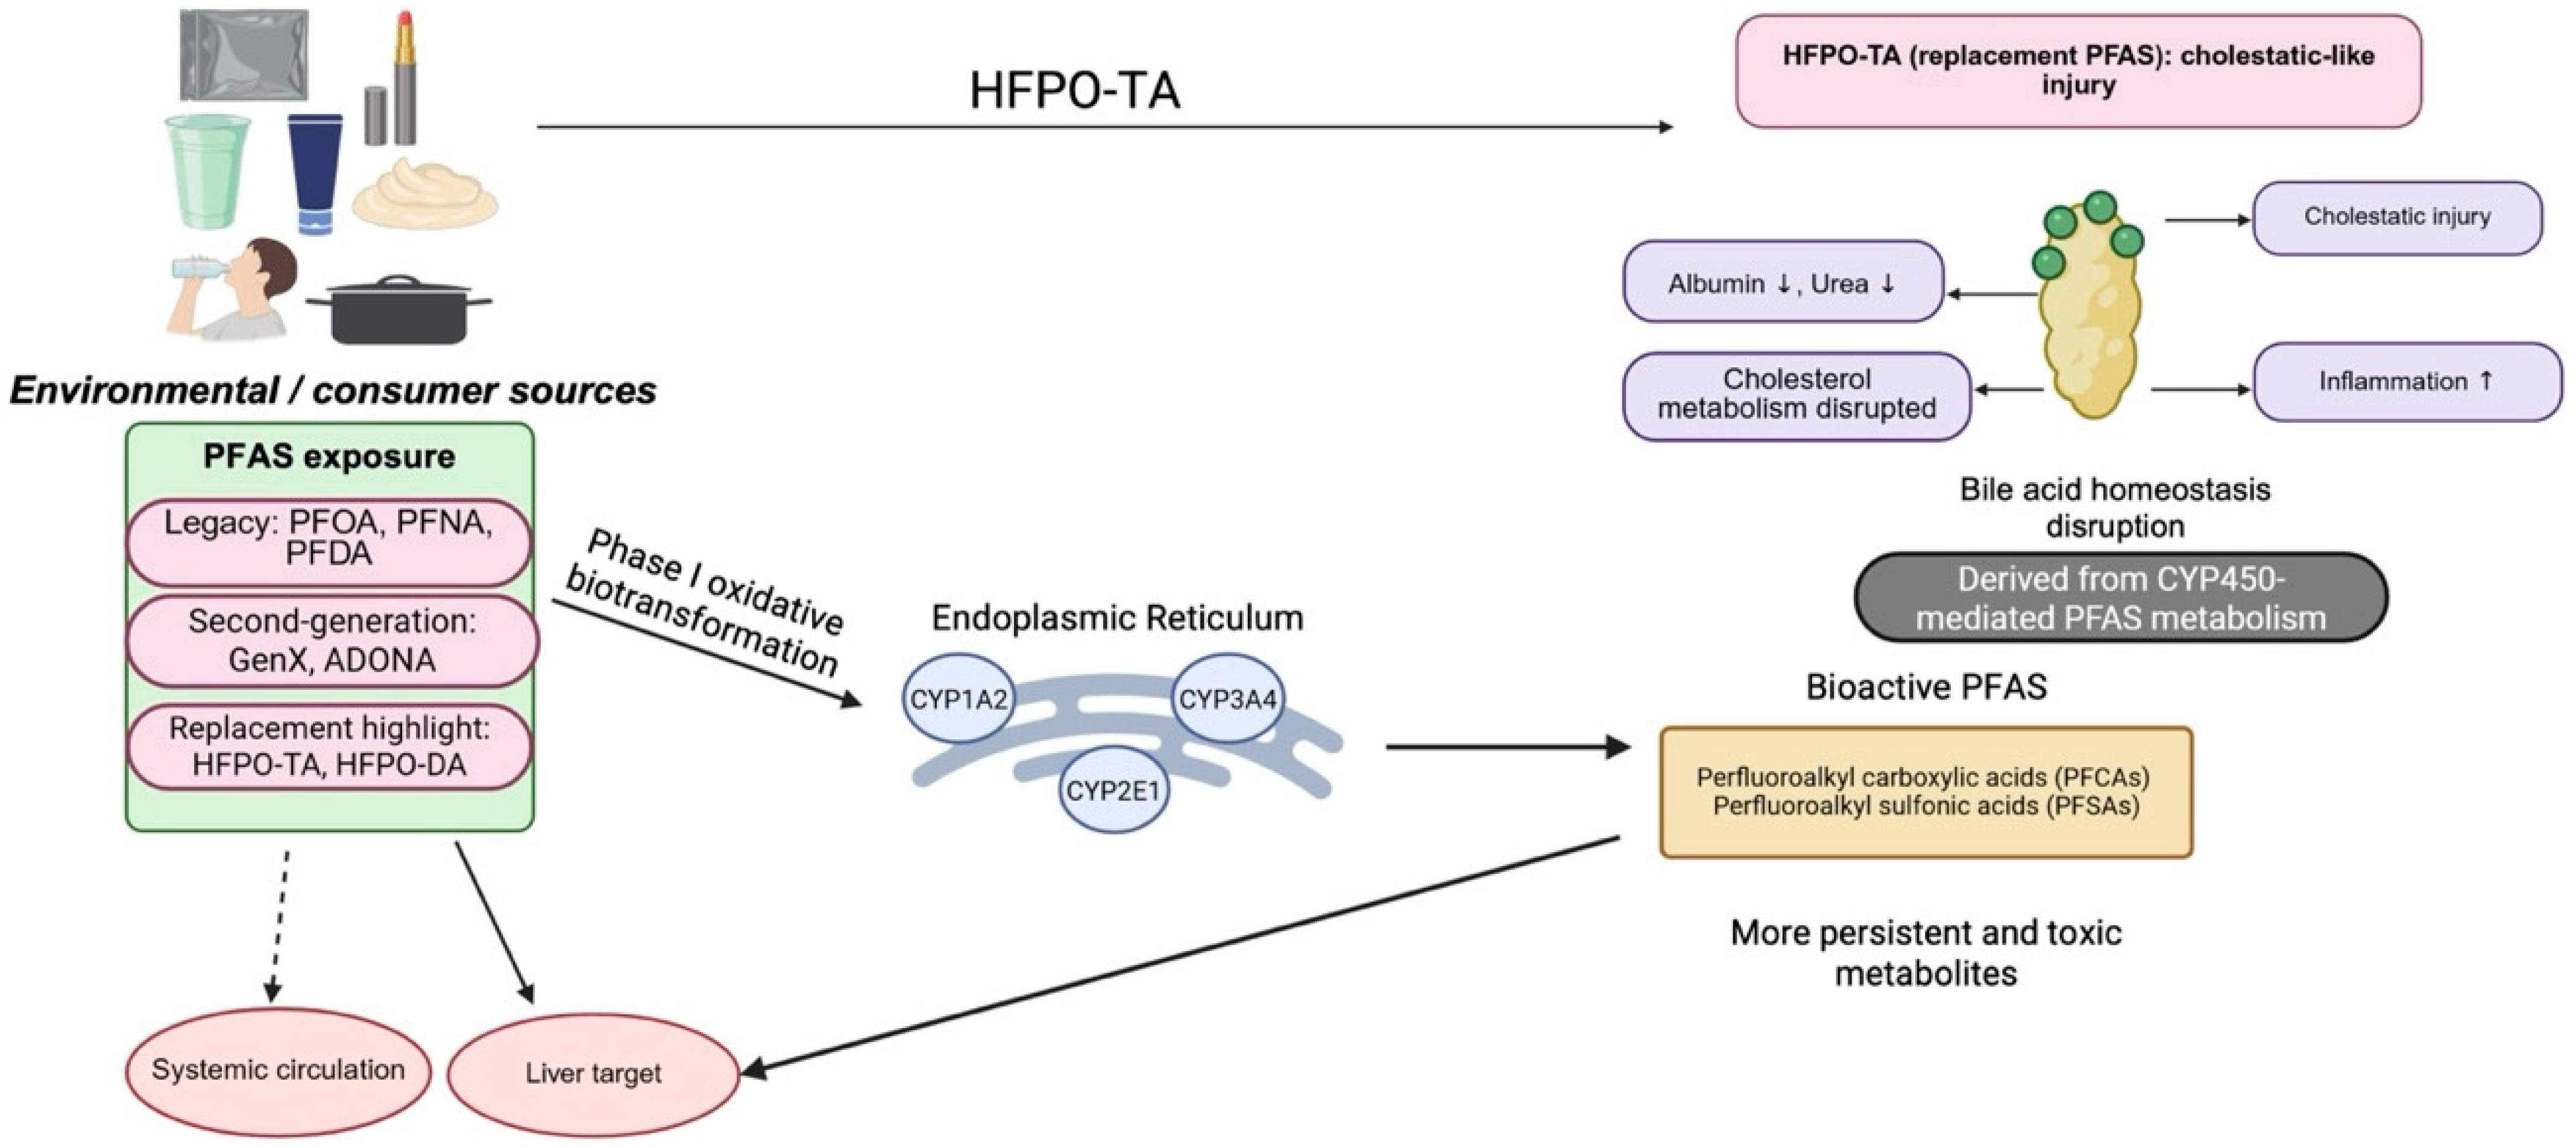
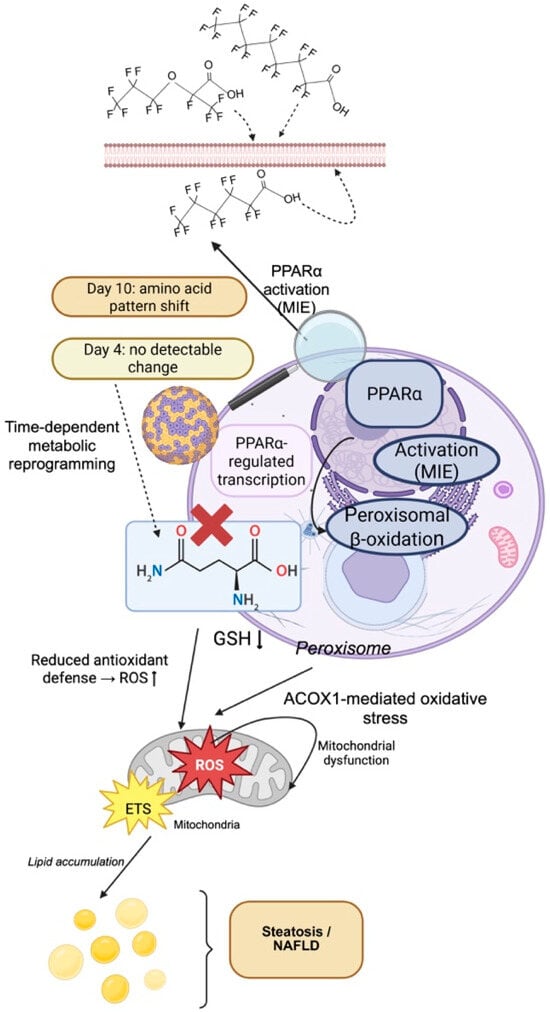
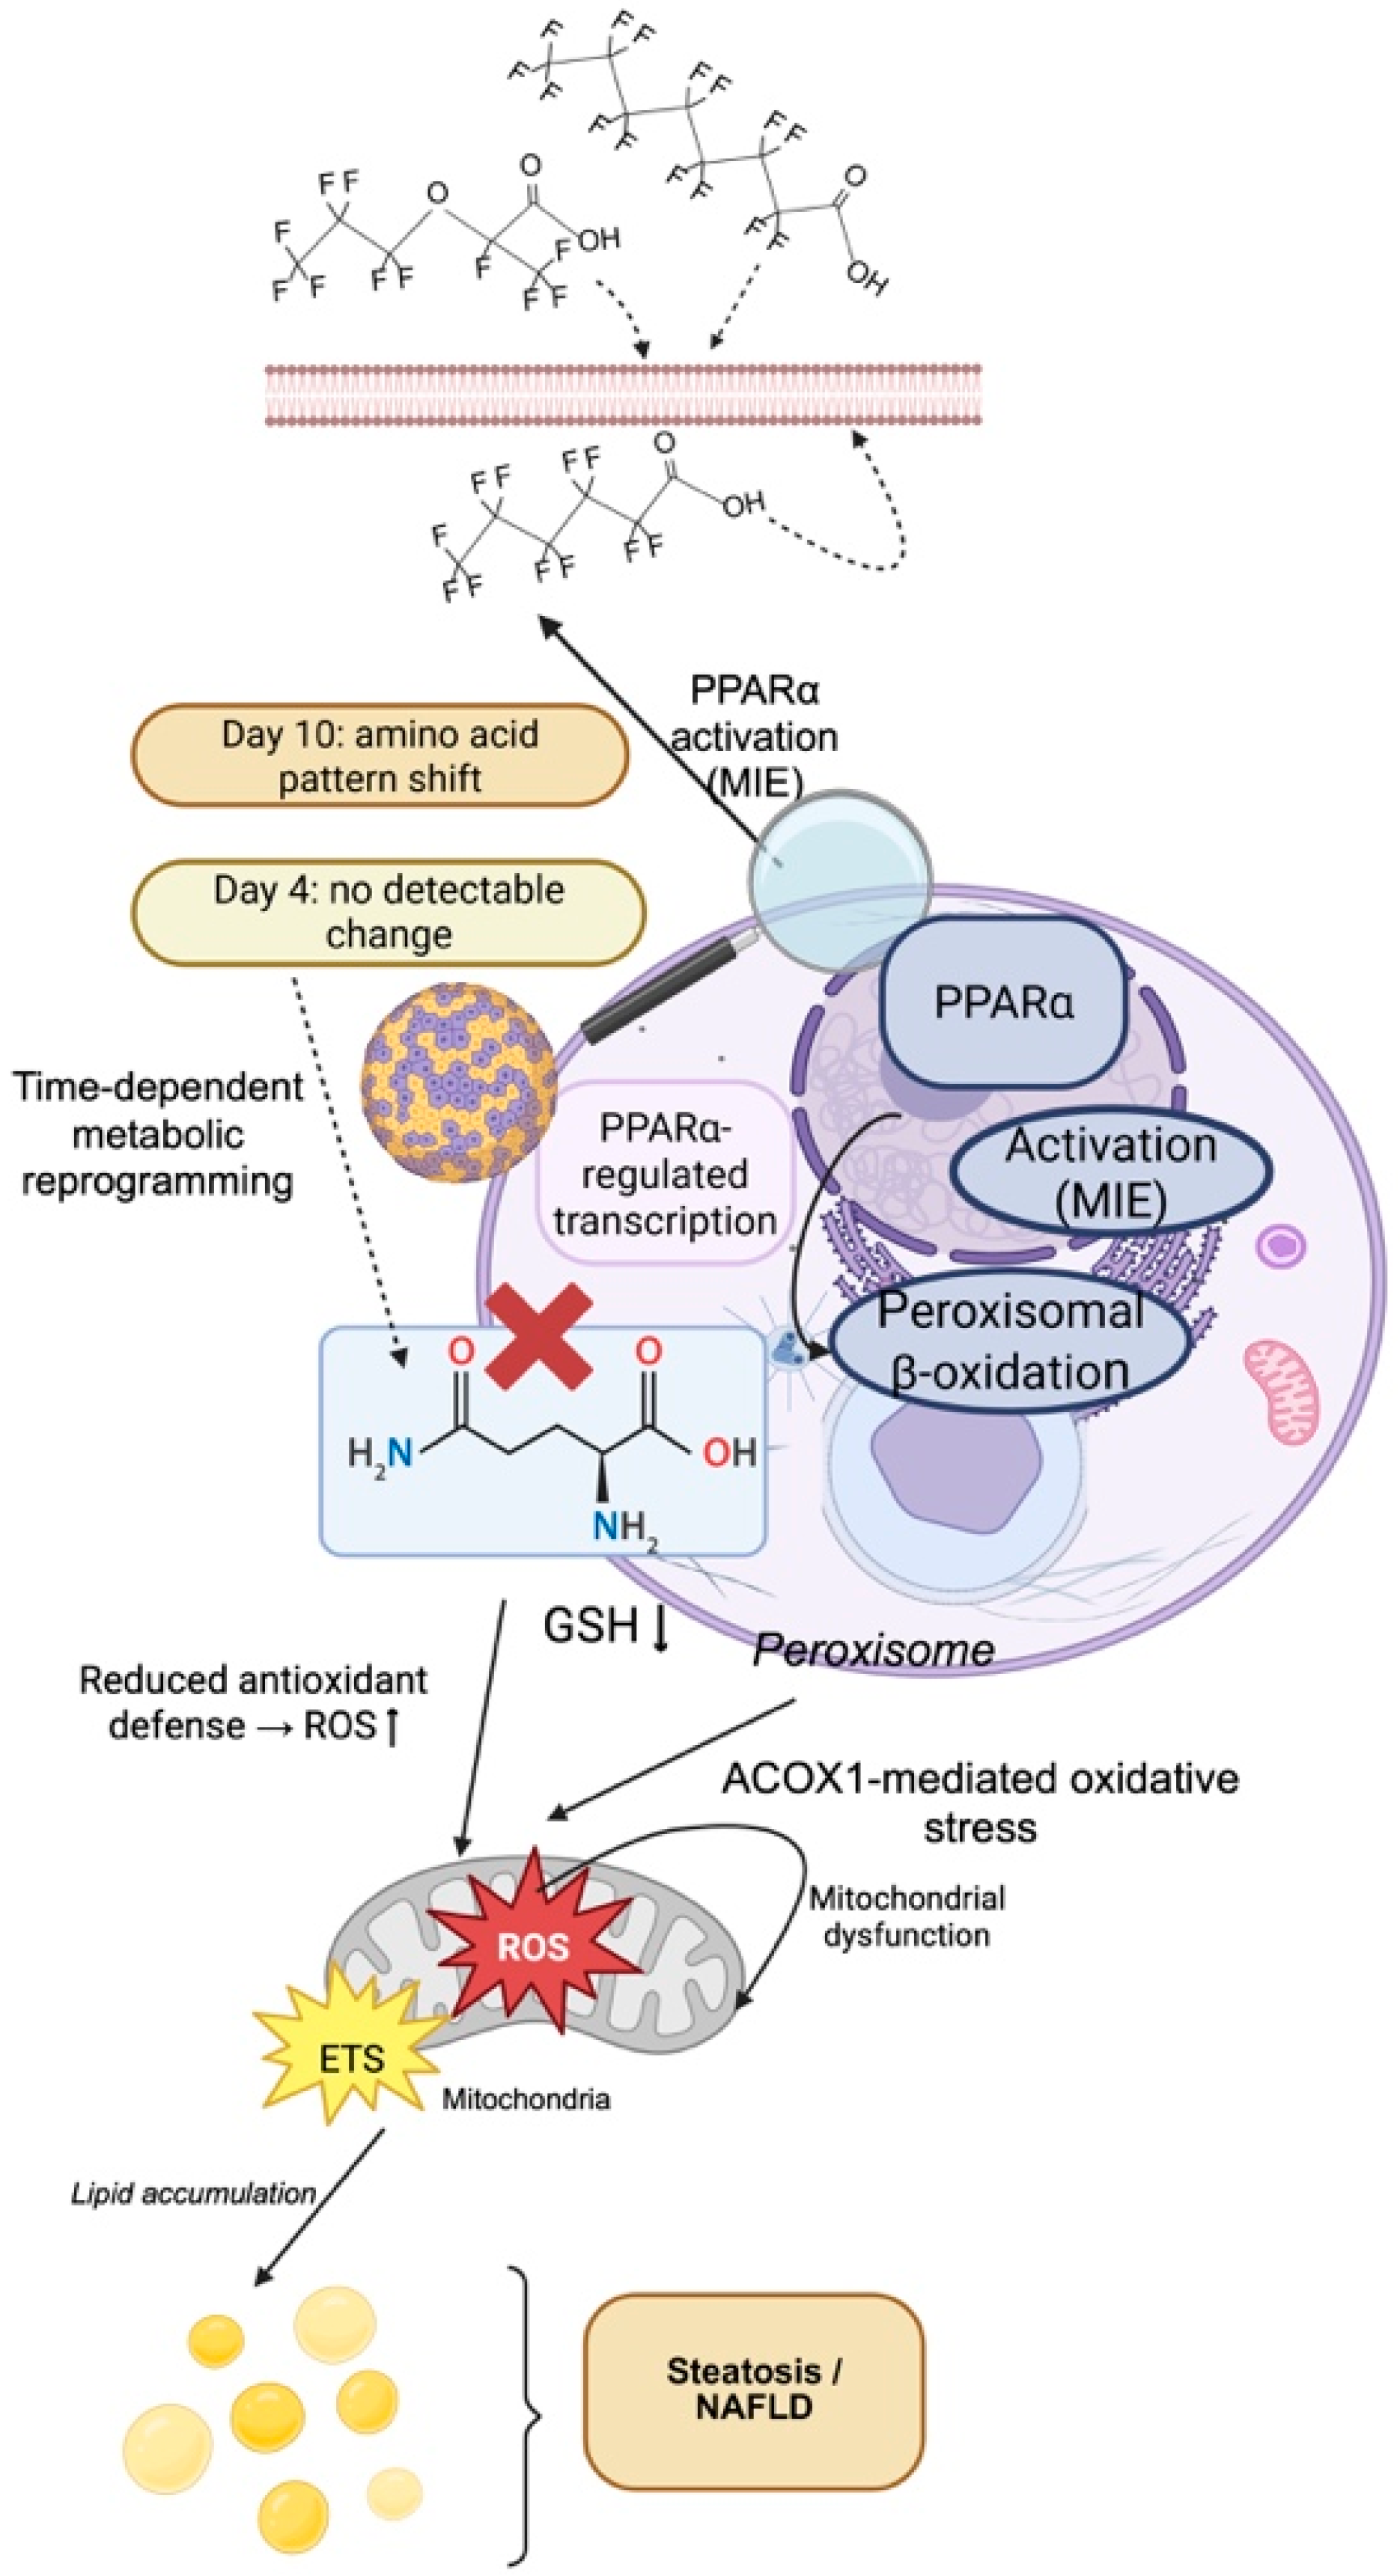

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.