


Abstract
Monascus yellow pigments, including monascin, ankaflavin, and the derivative monascinol, are azaphilone secondary metabolites produced by Monascus species. They have attracted attention as candidate functional-food ingredients because experimental studies indicate activity in pathways relevant to lipid and glucose metabolism. Available evidence, however, is heterogeneous and is derived predominantly from in vitro and animal studies; the human evidence is limited to small, short-term studies of Monascus-fermented preparations rather than isolated pigments. Reported associations with PPAR-α/γ and AMPK signaling, and with gut–liver-axis outcomes, should therefore be interpreted as mechanistic or preclinical observations. Monascus yellow pigments may offer a promising safety profile relative to monacolin K-containing preparations, but their long-term efficacy, dose standardization, and safety require confirmation in adequately powered human trials. Monascus-fermented products are being investigated beyond their traditional use as colorants and sources of monacolin K, partly because monacolin K has statin-like safety concerns. This review summarizes the structural diversity, biosynthetic pathways, and reported pharmacological activities of monascin, ankaflavin, and monascinol. Preclinical studies suggest that these azaphilones may influence PPAR-α/γ-, AMPK-, oxidative-stress-, and inflammation-related pathways and may affect lipid and glucose metabolism. Evidence for gut-microbiota modulation by monascinol is currently derived mainly from animal and mechanistic studies. Human data remain limited, including a small, short-duration trial of a Monascus-fermented preparation enriched in monascin and ankaflavin; these findings support short-term investigation but do not establish long-term clinical efficacy or comparative safety. Accordingly, Monascus yellow pigments should be regarded as promising candidate functional ingredients whose composition, bioavailability, dose, long-term safety, and clinical applicability require further rigorous evaluation.
1. Evolution of Monascus Fermentation from Traditional Colorants to Bioactive Yellow Pigments
1.1. Historical Background and Industrial Transition of Monascus Fermentation
Monascus species have been utilized in Asian food and pharmaceutical sectors for over a millennium, producing red, orange, and yellow pigments alongside pharmacologically active compounds such as monacolin K [1,2,3]. While industrial production historically favored Monascus red pigments, recent scientific focus has shifted toward Monascus yellow pigments because of their reported biological activities and physicochemical properties. In cellular and animal studies, monascin and ankaflavin have shown lipid-regulatory and anti-inflammatory effects with low observed toxicity under the tested conditions. However, direct, standardized comparisons of their efficacy and safety with monacolin K are limited, particularly in humans. Thus, monascin and ankaflavin are more appropriately described as promising functional-food components for further investigation than as established alternatives to lipid-lowering therapeutics [4,5].
Recent reviews also describe monascin and ankaflavin as central yellow-pigment metabolites with relevance to biosynthesis, production, pharmacology, and functional-food development [6,7].
1.2. Physicochemical Stability and Precision Fermentation Control
Monascus yellow pigments exhibit high physicochemical stability and can outperform red and orange pigments in their tolerance to light, thermal stress, and extreme pH, which enhances their commercial viability [8,9]. To further improve systemic bioavailability, recent research has successfully introduced nanoliposomal encapsulation to protect these pigments within the gastrointestinal tract [10]. Concurrently, precision fermentation has empowered researchers to manipulate secondary metabolic fluxes; for instance, the addition of calcium chloride (CaCl2) strongly upregulates the mppE gene, effectively redirecting biosynthesis toward the overproduction of yellow pigments [11]. Furthermore, utilizing specific nitrogen sources and optimizing pH levels can increase Monascus yellow pigment proportions while concurrently curtailing the generation of the mycotoxin citrinin [12]. This metabolic optimization addresses important safety bottlenecks, establishing a reliable foundation for toxin-free mass production [13].
1.3. Reported Multi-Target Molecular Activities
The biological relevance of Monascus yellow pigments stems from their multi-targeted molecular bioactivities. Natural monascin and ankaflavin have shown lipid-related, anti-inflammatory, and blood-pressure-related effects in experimental studies, including selective peroxisome proliferator-activated receptor modulation and activation of PPAR-α, PPAR-γ, and Nrf2-associated pathways [14]. Experimental studies have also reported effects on adipogenesis, lipid absorption, methylglyoxal-related stress, and oxidative-stress pathways [15,16,17]. These findings remain predominantly preclinical and should not be interpreted as established clinical efficacy.
1.4. Clinical Translational Evidence and Future Perspectives
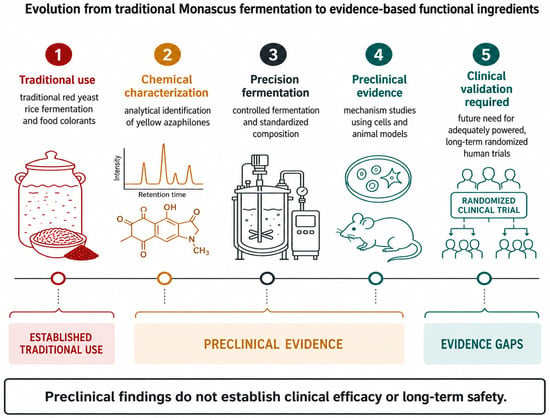
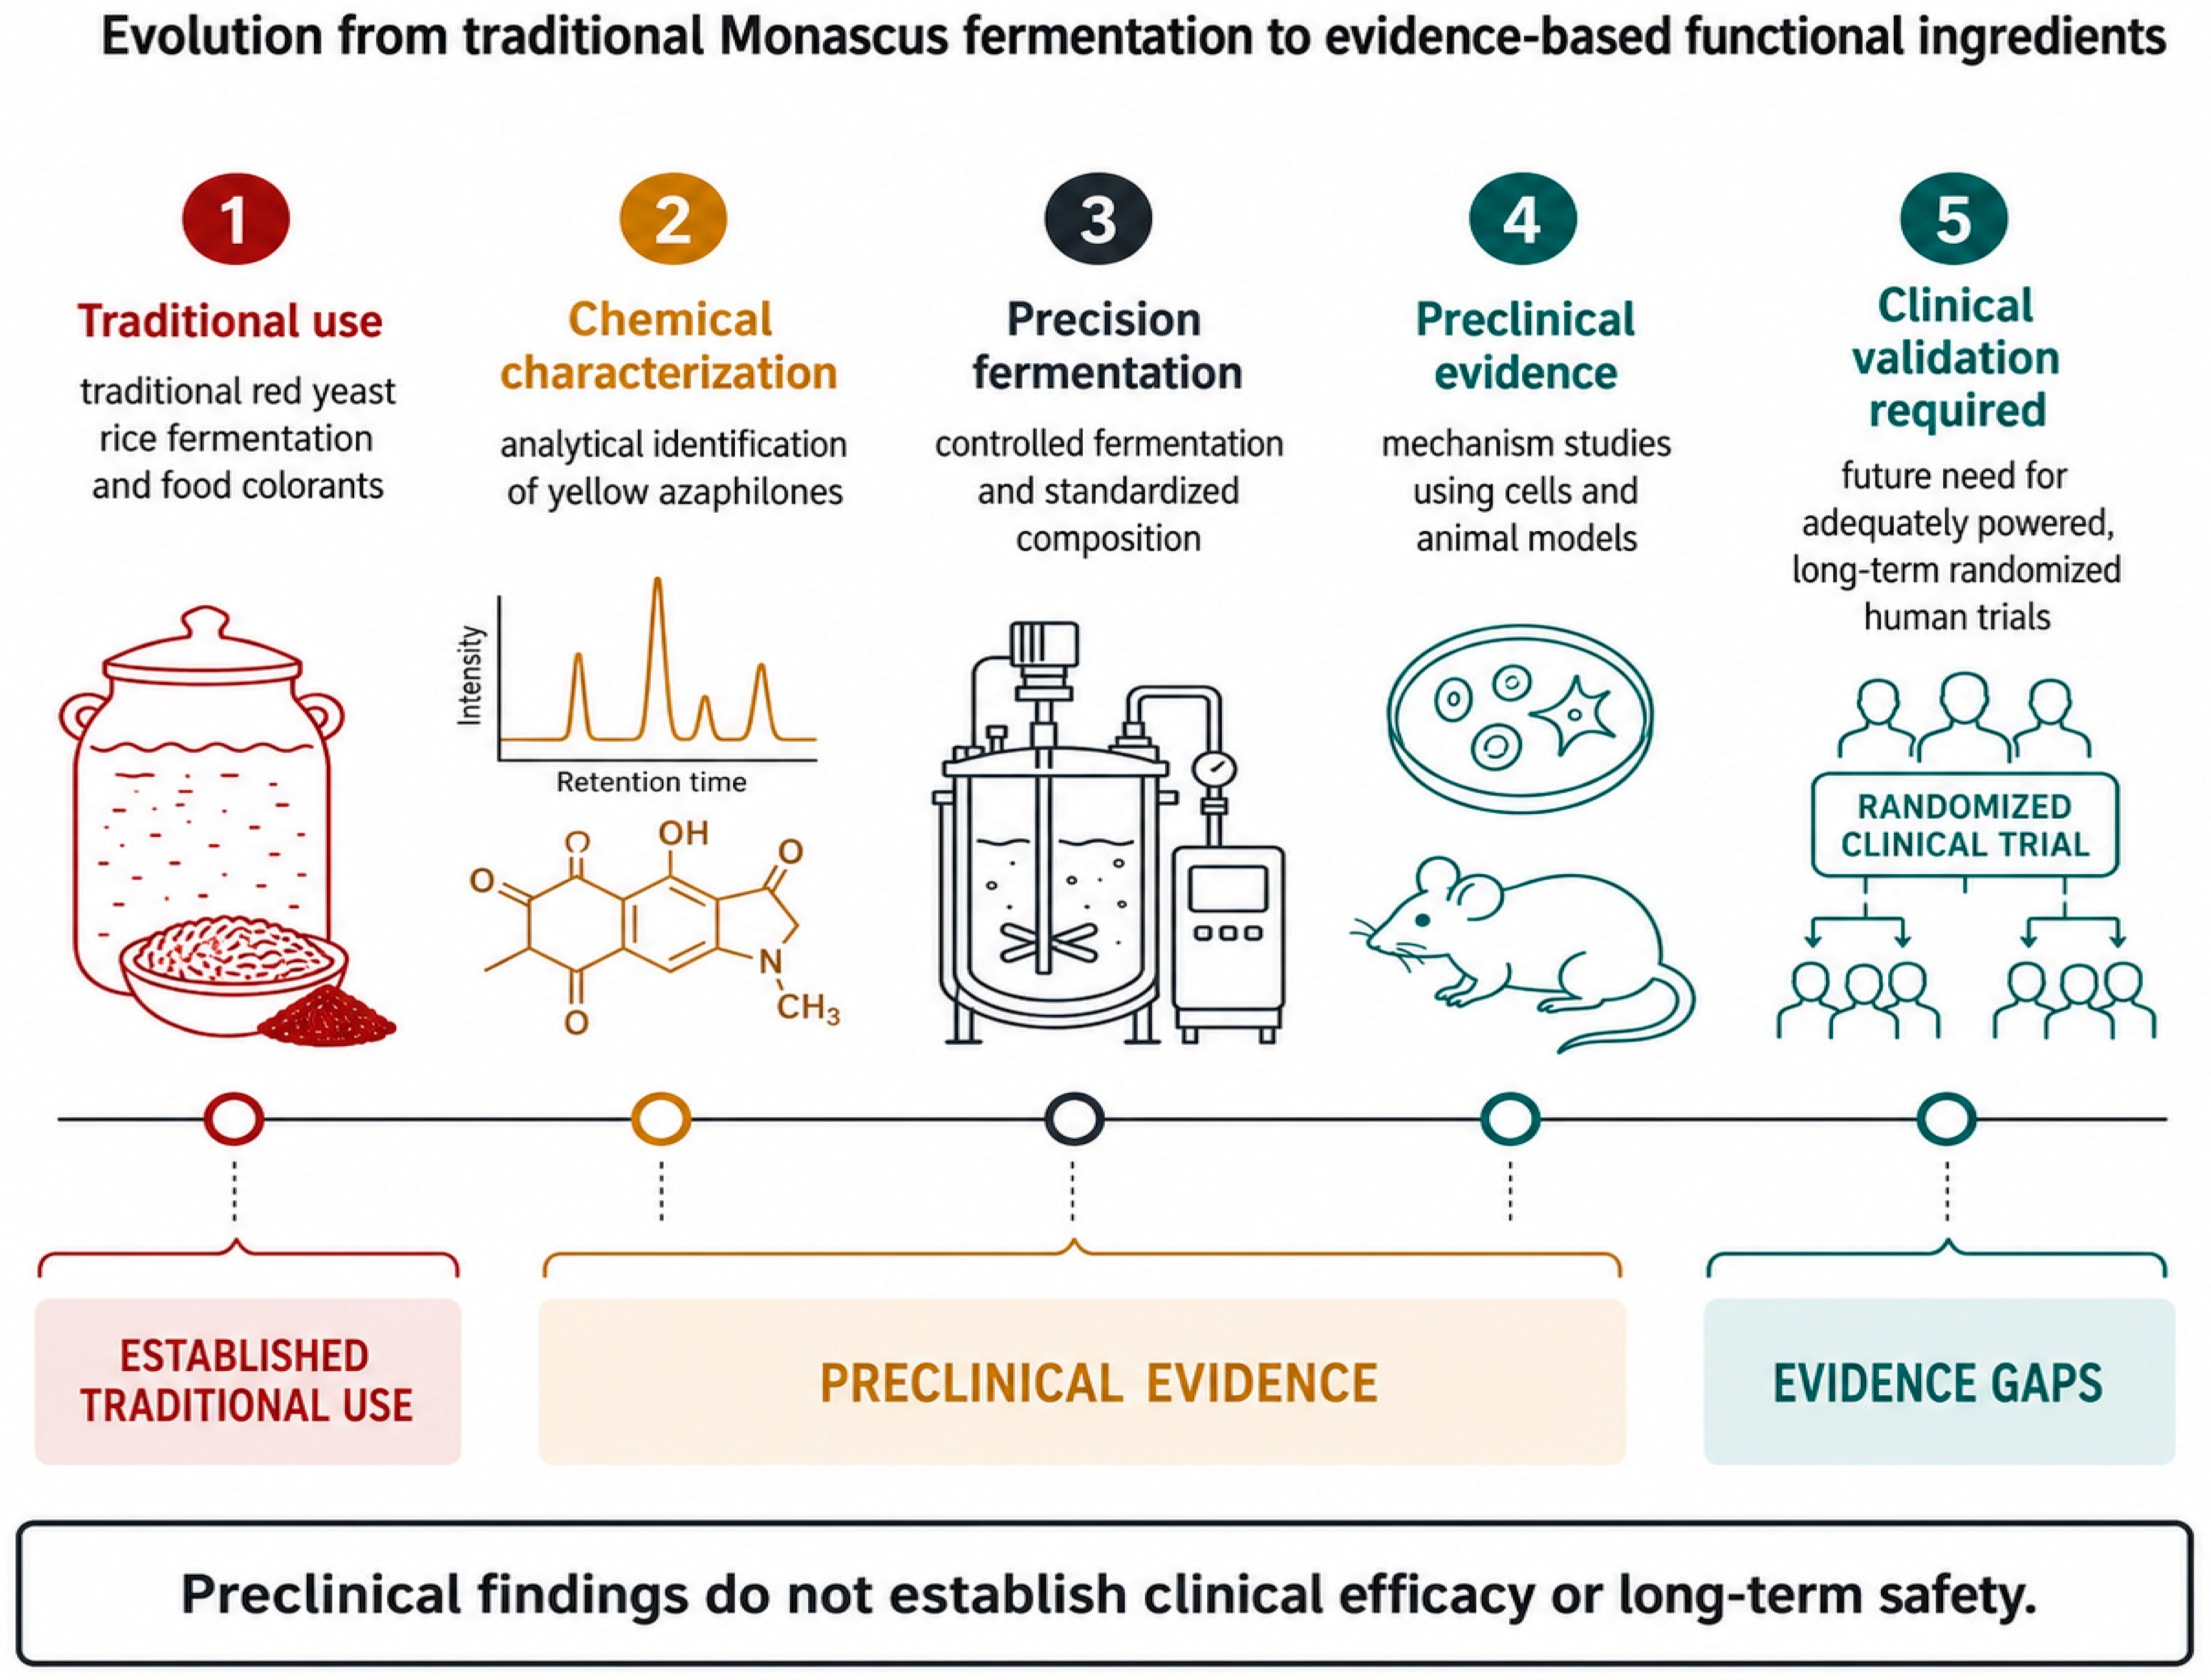
These preclinical mechanisms have begun to be explored in small human studies of complex Monascus-fermented preparations. In a randomized, double-blind study, an Ankascin 568 plus preparation was associated with improvements in blood-lipid measures over a short intervention period [5]. Because the available trial was small, short in duration, and did not test isolated monascin or ankaflavin, the findings should be interpreted as preliminary rather than as proof of efficacy or long-term safety for individual yellow pigments. Larger, longer, well-standardized clinical trials are required before therapeutic positioning or comparative claims can be made (Figure 1) [1].
Figure 1.
Evolution of Monascus fermentation from traditional colorants to bioactive yellow pigments based on published reviews, preclinical studies, and limited human evidence [1,2,3,4,5].
2. Chemical Identity and Diversity: Structures of Monascin, Ankaflavin, and the Derivative Monascinol
2.1. Monascus-Produced Yellow Pigments
Pigments produced by Monascus species are a major class of fungal secondary metabolites with significant chemical diversity and biological activity [18]. Among these, monascin and ankaflavin are the principal yellow azaphilone pigments, while monascinol is a structurally related derivative. These compounds are biosynthesized via polyketide pathways and share a common azaphilone core structure, which is responsible for their distinct chromophoric characteristics and high chemical reactivity. With advancements in analytical chemistry, researchers have isolated and elucidated the precise structural characteristics of these yellow pigments from extracts of Monascus pilosus and Monascus purpureus using two-dimensional nuclear magnetic resonance (2D NMR) and spectral analysis [19,20]. The chemical identification and quantification of these pigments require validated analytical methods appropriate to complex fermentation matrices.
Additional analytical studies have strengthened the chemical characterization of Monascus yellow pigments through separation and identification of yellow/orange pigment fractions and water-soluble derivatives [21,22].
Monascin is a typical azaphilone compound characterized by a highly oxygenated bicyclic (pyranoquinone) core. It contains hydroxyl and carbonyl functional groups, possesses a relatively shorter alkyl side chain, and displays moderate polarity. Monascin has the chemical formula C21H26O5, and its crystal structure belongs to the orthorhombic P212121 space group [23]. Single-crystal X-ray diffraction and Hirshfeld surface analysis indicate that intermolecular C-H...O hydrogen bonds play a key role in maintaining its 2D and 3D network structures. Furthermore, molecular electrostatic potential (MEP) mapping reveals that four oxygen atom regions within the monascin molecule possess strong negative charges, which act as preferential binding sites for positively charged amino acid residues during molecular recognition.
Ankaflavin shares the same azaphilone backbone and chromophore core as monascin, but it differs structurally by having a longer hydrophobic alkyl side chain. This variance significantly increases its lipophilicity, which consequently alters its interactions with cellular membranes. In the Monascus fermentation process, monascin and ankaflavin are typically co-produced as the major yellow pigments [18,23,24].
Monascinol is a reduced derivative of monascin that differs principally in the oxidation state of its functional groups. Although it retains the azaphilone core scaffold, biological activity can differ across assays and should not be interpreted as a therapeutic ranking. The Monascus genus also shows substantial metabolite diversity: monascin and novel azaphilone pigments, including Monascusone A and B, have been isolated from a yellow mutant of Monascus kaoliang [25]. Studies of purified Monascus pigments likewise report that related derivative series display different bioactivities in experimental systems [26]. A detailed summary of the chemical identity and structure–activity considerations of major pigments is presented in Table 1.
Table 1.
Chemical identity and structure–activity relationships of Monascus yellow pigments.
2.2. Structural Diversity and Structure–Function Relationship
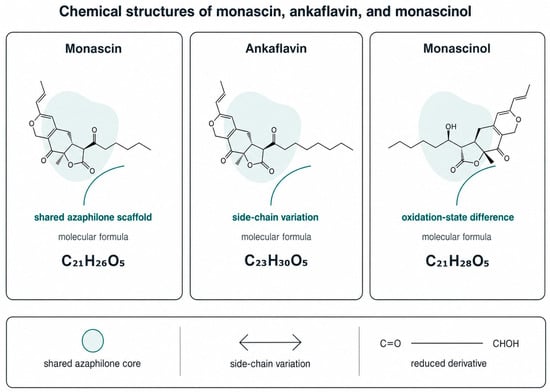
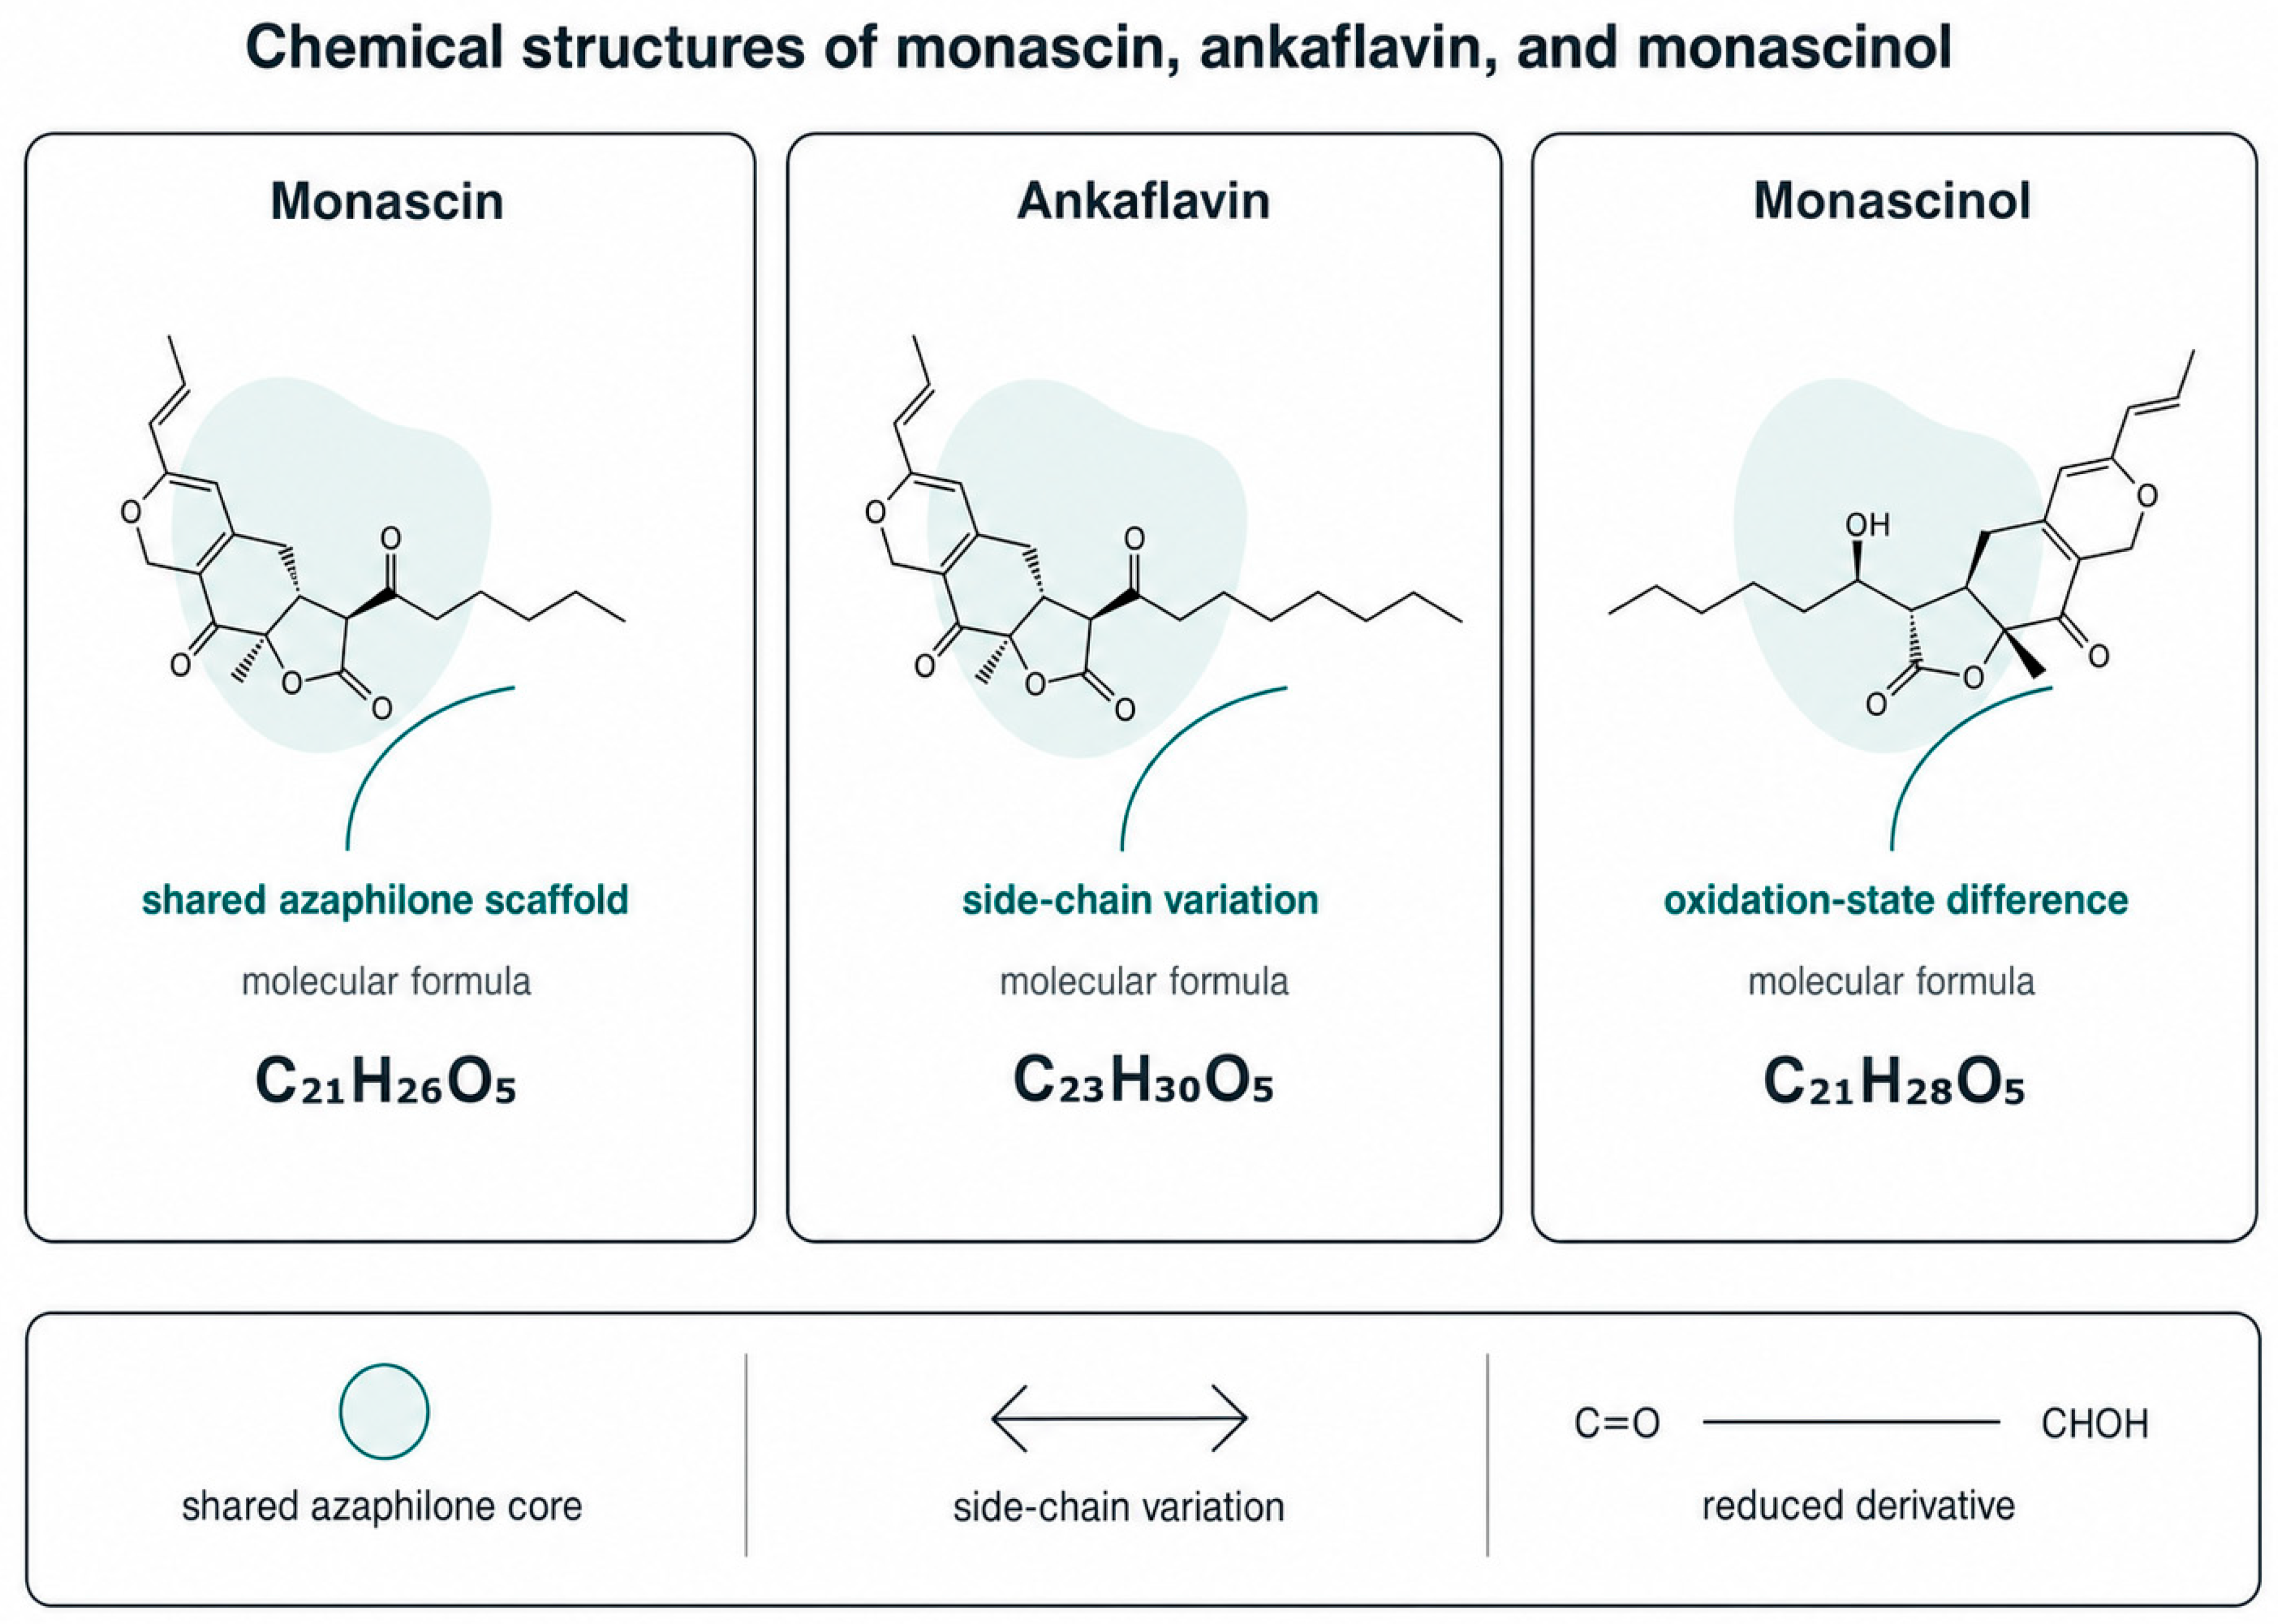
The shared azaphilone scaffold and variations in side-chain length or oxidation state are associated with differences in physicochemical properties and experimental bioactivities. Direct comparisons across assays and models should not be interpreted as a therapeutic ranking. The representative structures are shown in Figure 2. For example, ankaflavin showed selective cytotoxicity in Hep G2 cells in one experimental study [24]. In cellular and animal studies, monascin and ankaflavin have been associated with reduced adipogenesis, altered lipid-related pathways, and inhibition of intestinal Niemann–Pick C1-Like 1 (NPC1L1) [15,27]. These preclinical observations do not establish efficacy equivalent to monacolin K in humans. Short-term studies of complex fermented preparations have not reported major safety signals under the conditions tested, but this does not establish long-term safety for isolated pigments [5].
Figure 2.
Representative chemical structures of monascin, ankaflavin, and monascinol. Created by the authors based on published structural and chemical-characterization studies [18,23,24,25,26].
Monascin, ankaflavin, and their derivative monascinol represent a group of structurally related azaphilone compounds characterized by a shared chemical backbone. Precise variations in alkyl side chains and oxidation states yield significant differences in their physicochemical properties and biological activities. Current academic research has developed efficient methods for their structural identification and analysis, supporting further investigation of their possible roles in pathways relevant to cardiovascular and metabolic health. These findings underscore the core role of structural diversity in determining the functional capabilities of Monascus yellow pigments. As the research focus shifts from basic structural identification to in-depth profiling of molecular mechanisms, future studies that explore the pharmacological mechanisms and structure–activity relationships (SAR) of derivatives such as monascinol will be critical for advancing the development of natural functional-food ingredients [18,26].
2.3. Broader Yellow-Pigment Diversity, Analytical Characterization, and Structure–Activity Considerations
The term Monascus yellow pigments encompasses more than monascin, ankaflavin, and monascinol. The reported chemical space includes lipophilic and water-soluble azaphilone derivatives, compounds differing in side-chain length or oxidation state, and pigment–amine adducts generated under particular fermentation conditions. Their occurrence depends on strain background, culture conditions, precursor availability, and downstream processing. Accordingly, chemical identity should be established for each preparation rather than inferred from color alone [1,7,8,9,21,22].
Chromatographic separation coupled with photodiode-array detection, high-resolution mass spectrometry, and, where feasible, NMR confirmation provides complementary information on pigment identity, relative composition, and structural isomers. For functional-food development, a practical analytical specification should quantify the intended marker compounds and screen for monacolin K and citrinin, while also documenting extraction method, batch variability, and storage conditions. Such reporting is essential for relating a biological result to a defined material [21,22,28].
Current structure–activity evidence is strongest for qualitative relationships: longer or more hydrophobic side chains may alter lipophilicity and interactions with model systems, whereas changes in oxidation state and functional groups may influence chemical reactivity. However, direct evidence linking specific structural changes to human absorption, membrane permeability, receptor binding, metabolism, or clinical efficacy remains limited. Structure–activity discussion should therefore be interpreted as a research framework rather than as a basis for therapeutic ranking [18,26] (Table 2).
Table 2.
Practical classification and analytical considerations for selected Monascus yellow-pigment groups.
3. Biosynthetic Pathways: Molecular Mechanisms of Azaphilone Synthesis in Monascus Species
3.1. Biosynthetic Gene Cluster and Core Enzymatic Machinery
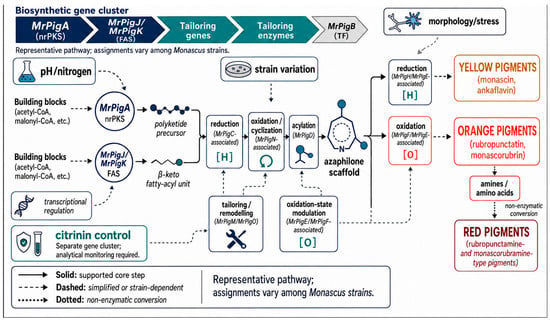
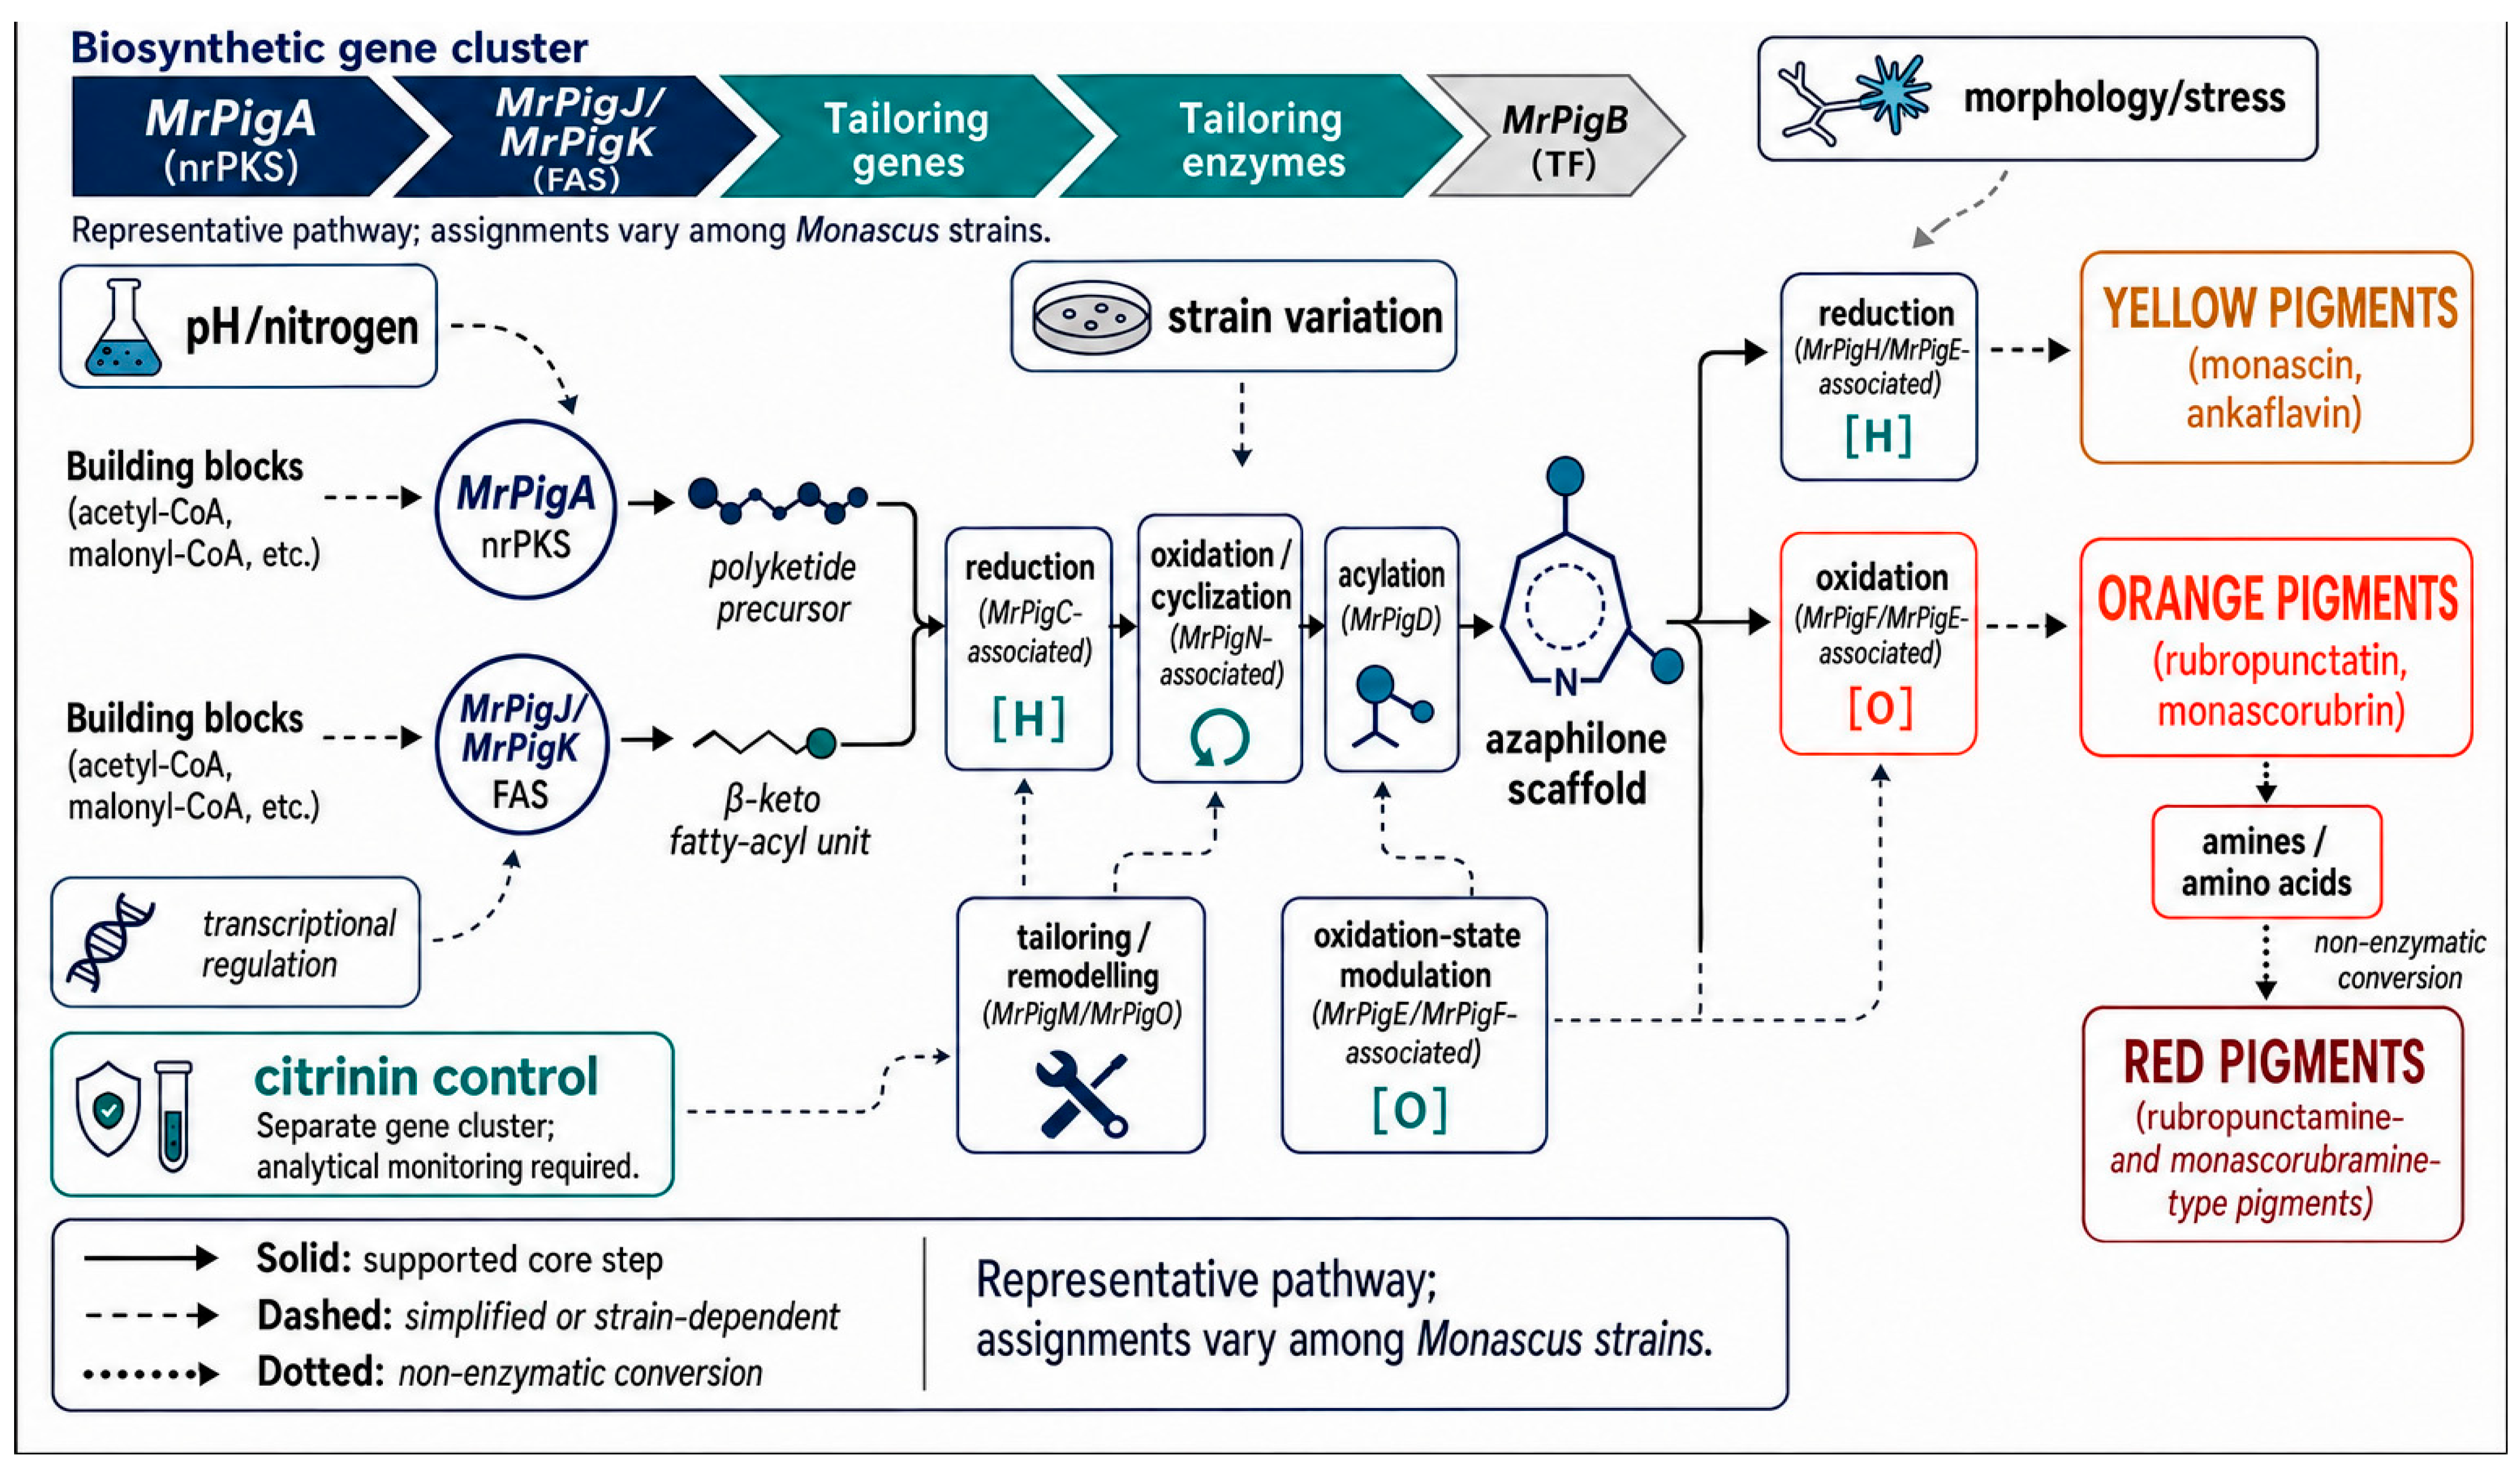
The biosynthesis of Monascus azaphilone pigments is directed by a specialized biosynthetic gene cluster (BGC), experimentally delimited from mrpigA to mrpigP [29,30]. At the core of this pathway is a non-reducing polyketide synthase (nrPKS) that constructs the pyranoquinone bicyclic scaffold, while a dedicated fatty acid synthase (FAS) supplies short-chain fatty-acyl moieties for side-chain decoration [31,32]. Together, these coordinated enzymatic steps generate the structural diversity of Monascus azaphilone pigments.
3.2. Stepwise Formation of Yellow, Orange, and Red Azaphilones
Azaphilone scaffold diversification occurs through a branched pathway involving sequential reduction, oxidation, and acylation reactions [33,34,35]. The reductive branch, predominantly involving the mppE gene, is required for synthesizing yellow pigments such as monascin and ankaflavin, whereas oxidative tailoring governed by the mppG oxidase gene produces orange pigments [36]. Inactivating mppG selectively abolishes orange pigments while preserving yellow ones, indicating that they arise from diverging branches rather than simple linear conversion [36]. Furthermore, major red azaphilones are often generated non-enzymatically when orange intermediates react spontaneously with amine-containing compounds, significantly expanding the pigment spectrum established by the primary biosynthetic machinery [37].
3.3. Metabolic Flux and Precursor Supply
The supply of primary metabolites from the tricarboxylic acid (TCA) cycle and glycolysis is vital for determining overall pigment yield [38,39,40]. While protein S-nitrosylation inhibits TCA-cycle enzymes and restricts pigment synthesis [38], supplementing cultures with isopropyl myristate, extractive fermentation, and oxidoreduction-potential control provide process strategies for improving yellow-pigment output [41,42].
Beyond precursor supply, liquid-culture studies show that fermentation conditions, high-glucose stress, and integrated culture systems can alter mycelial morphology and improve yellow pigment production [43,44,45].
3.4. Genetic and Epigenetic Regulation
Genetic and epigenetic factors play a central regulatory role in secondary metabolism [46]. Modern molecular techniques have identified specific regulators, such as the VeA gene, whose deletion completely halts both pigment and citrinin production; transcriptomic, epigenetic, and gene-cluster studies further clarify how pigment, citrinin, and monacolin pathways are co-regulated [46,47,48,49]. Epigenetic modifications also significantly affect pathway activation; altering histone acetylation via inhibitors or targeted deletion of specific genes can selectively suppress the citrinin pathway [50,51].
Comparative transcriptional and gene-function studies further indicate that pigment diversity is strongly shaped by transcriptional regulation and that citrinin-linked genes such as ctnF and ctnA influence both toxin control and pigment production [52,53,54].
3.5. Production, Standardization, and Quality-Control Considerations
Production of yellow pigments should be evaluated as an integrated strain–process–product system. Reported approaches include selection of low-citrinin isolates, adjustment of nitrogen source and pH, control of culture morphology and stress conditions, and genetic or mutagenesis-based strain improvement. These approaches can increase yellow-pigment yield or alter pigment composition, but results are strain- and process-specific and should not be generalized without compositional verification [7,11,12,28,52,55,56,57,58,59,60,61,62,63,64,65].
For translation into foods or supplements, each batch should be characterized for marker-pigment composition, residual citrinin, monacolin K content, microbial and chemical contaminants, and storage stability under the intended formulation conditions. Batch release criteria should be linked to validated analytical methods and should include acceptance ranges for the intended active markers. Because fermentation products may differ substantially between strains and processing methods, evidence obtained with one standardized extract cannot automatically be transferred to another product [28,66].
Regulatory positioning depends on jurisdiction, product composition, intended use, dose, and claims. The review therefore does not assume that a pigment-rich preparation is inherently approvable as a functional food or pharmaceutical ingredient. Early development should integrate safety testing, compositional control, and claim substantiation with the applicable regulatory pathway [28,66,67,68].
3.6. Environmental Stress, Compartmentalization, and Pathway Branching
Azaphilone synthesis is spatially organized and responsive to environmental stressors, with specific biosynthetic enzymes compartmentalized across the mitochondria, cytosol, and cell wall [69]. External elicitors such as acidic stress, silicon dioxide (SiO2) microparticles, nitrate supplementation, temperature shifts, food-grade modifiers, and organic nitrogen sources can alter yellow-pigment output and mycelial morphology [26,55,56,57,58,59,60,61,70]. These observations support the use of controlled cultivation conditions as a practical strategy for optimizing pigment production and limiting undesired by-products.
From a quality-control perspective, isolate selection and citrinin-reduction strategies remain essential because Monascus strains vary substantially in citrinin occurrence, detection, and reduction during red fermented rice production [28].
Process-oriented studies also show that nitrate addition, pH/nitrogen balance, and taurine-mediated transcriptional and membrane effects can reshape Monascus pigment output and related fermentation behavior [60,61,66].
In Monascus species, azaphilone biosynthesis is a sophisticated network controlled by a specialized BGC featuring an nrPKS and a dedicated FAS [29,71]. Recent advances highlight the value of multi-omics, epigenetic regulation, and metabolic-flux engineering for investigating pigment production [31,69]. These approaches may support targeted production while minimizing citrinin contamination, subject to compositional, safety, and regulatory evaluation. The integrated mechanisms and key components regulating Monascus azaphilone biosynthesis are summarized in Table 3 and Figure 3.
Table 3.
Integrated mechanisms regulating Monascus azaphilone biosynthesis.
Figure 3.
Simplified biosynthetic framework for Monascus azaphilone pigments. Created by the authors based on reported gene-cluster, scaffold-assembly, enzymatic, and pathway-branching studies [29,31,32,33].
4. Reported Effects on Lipid Metabolism: Preclinical and Limited Human Evidence
Secondary metabolites derived from Monascus fermentation, particularly the yellow azaphilone pigments monascin and ankaflavin, have been investigated for possible roles in lipid metabolism and metabolic disease. The evidence base includes in vitro mechanistic studies and animal models, with limited human studies of Monascus-fermented preparations. These data support further evaluation of lipid-regulatory and anti-inflammatory mechanisms, but they do not yet establish clinical efficacy for preventing or treating metabolic syndrome or non-alcoholic fatty liver disease (NAFLD) [4,5,14,15].
4.1. Core Regulatory Mechanisms: PPAR Signaling and AMPK Activation
A central mechanism underlying the reported lipid-regulating activity of monascin and ankaflavin is their function as natural modulators of peroxisome proliferator-activated receptors (PPARs) and their synergistic activation of AMP-activated protein kinase (AMPK). In murine models of NAFLD, monascin and ankaflavin have been shown to act as specific peroxisome proliferator-activated receptor alpha (PPAR-α) agonists and AMPK activators, thereby suppressing hepatic fatty acid uptake and lipogenesis while significantly promoting fatty acid β-oxidation [14]. These molecular actions lead to a marked reduction in plasma levels of total cholesterol (TC), triglycerides (TG), free fatty acids (FFA), and low-density lipoprotein cholesterol (LDL-C). Furthermore, this process is accompanied by the upregulation of farnesoid X receptor (FXR) and peroxisome proliferator-activated receptor-gamma coactivator 1-alpha (PGC-1α), supporting a possible hepatoprotective effect in the cited animal models. Beyond PPAR-α, monascin and ankaflavin also have been reported to modulate the peroxisome proliferator-activated receptor gamma (PPAR-γ) pathway [15]. In fructose-induced obese and diabetic mouse models, monascin functions as an effective PPAR-γ agonist that significantly improves insulin sensitivity, ameliorates hyperglycemia and hyperinsulinemia, and downregulates lipogenic transcription factors, including sterol regulatory element-binding protein-1c (SREBP-1c) and carbohydrate-responsive element-binding protein (ChREBP). The reliance on this specific metabolic pathway was further corroborated when the administration of a PPAR-γ antagonist explicitly blunted these anti-lipogenic and hypoglycemic benefits, confirming the targeted receptor dependency [15].
4.2. Lipoprotein Assembly and Intestinal Absorption Modulation: Apo A1 and NPC1L1
In addition to nuclear receptor signaling, the hypolipidemic efficacy of monascin and ankaflavin is profoundly mediated through the regulation of apolipoprotein expression and the suppression of intestinal lipid absorption; independent pigment studies also support broader metabolic effects in high-fat-diet models [72]. A critical regulatory target is apolipoprotein A1 (Apo A1), the primary structural component of high-density lipoprotein (HDL) [73]. Experimental evidence indicates that monascin and ankaflavin significantly stimulate the hepatic expression of Apo A1, thereby promoting HDL formation and enhancing reverse cholesterol transport, which accelerates the efflux of cholesterol from peripheral tissues. Concurrently, these azaphilone compounds suppress the assembly of low-density lipoproteins, effectively reducing LDL-C accumulation while maintaining or even elevating HDL levels to restore systemic lipoprotein homeostasis [4,26]. In the context of anti-obesity mechanisms, monascin and ankaflavin actively inhibit the expression of CCAAT/enhancer-binding protein beta (C/EBPβ) and its downstream targets, PPAR-γ and CCAAT/enhancer-binding protein alpha (C/EBPα), thereby effectively blocking the early differentiation of preadipocytes and subsequent lipid accumulation. Furthermore, these compounds directly downregulate the expression of Niemann-Pick C1-Like 1 (NPC1L1) protein in the small intestine, efficiently curtailing the absorption of exogenous lipids at the gastrointestinal source [15].
4.3. Antioxidant and Anti-Inflammatory Efficacy in Disease Models
Animal models provide preclinical evidence that monascin and ankaflavin may influence inflammatory and oxidative-stress pathways, while independent studies of Monascus yellow pigments report antioxidant and protein-protective effects in biochemical models [74,75,76]. These findings support further mechanistic investigation but do not by themselves establish clinical efficacy or therapeutic value.
Complementary formulation and protein-interaction studies broaden this evidence base by examining Monascus yellow pigment delivery systems and ankaflavin/monascin interactions with amyloidogenic protein models [77,78].
4.4. Limited Human Evidence and Safety Considerations
Clinical evaluation of Monascus purpureus NTU 568-derived functional extracts has focused particularly on preparations enriched with monascin and ankaflavin. A 12-week randomized, double-blind, placebo-controlled clinical trial evaluated the efficacy of Ankascin 568 plus in 40 subjects presenting with borderline hypercholesterolemia characterized by elevated TC and LDL-C levels [5]. Following daily supplementation with 500 mg of the extract for 4 weeks, TC levels decreased by 11.9%, and LDL-C was reduced by 19.0% compared with baseline. Monitoring of hepatic, renal, and thyroid functions, glycemic indices, and CPK activity supported the short-term tolerability of the extract. The absence of abnormal CPK elevation is clinically relevant because monacolin K, as a statin-like compound, is associated with muscle-toxicity concerns. These findings support the potential of monascin- and ankaflavin-rich preparations as lipid-regulating functional ingredients, although additional larger and longer-term human studies remain necessary.
In summary, monascin and ankaflavin have been reported to influence Apo A1-related lipoprotein biology, PPAR- and AMPK-associated signaling, and pathways involved in lipid absorption (Table 4). The strength of support differs by endpoint: mechanistic evidence is largely cellular, efficacy evidence is primarily preclinical, and human observations are limited to small studies of complex Monascus preparations. These compounds therefore warrant further study as candidate functional ingredients, while their long-term safety, effective dose range, composition-dependent effects, and clinical relevance remain to be established [5,14,15,73].
Table 4.
Summary of lipid metabolism regulation by Monascus yellow pigments.
5. Reported Effects on Glucose Homeostasis and Pancreatic Cell Models
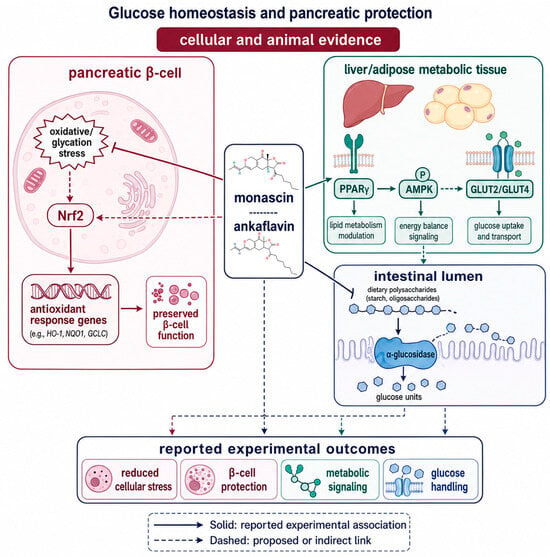
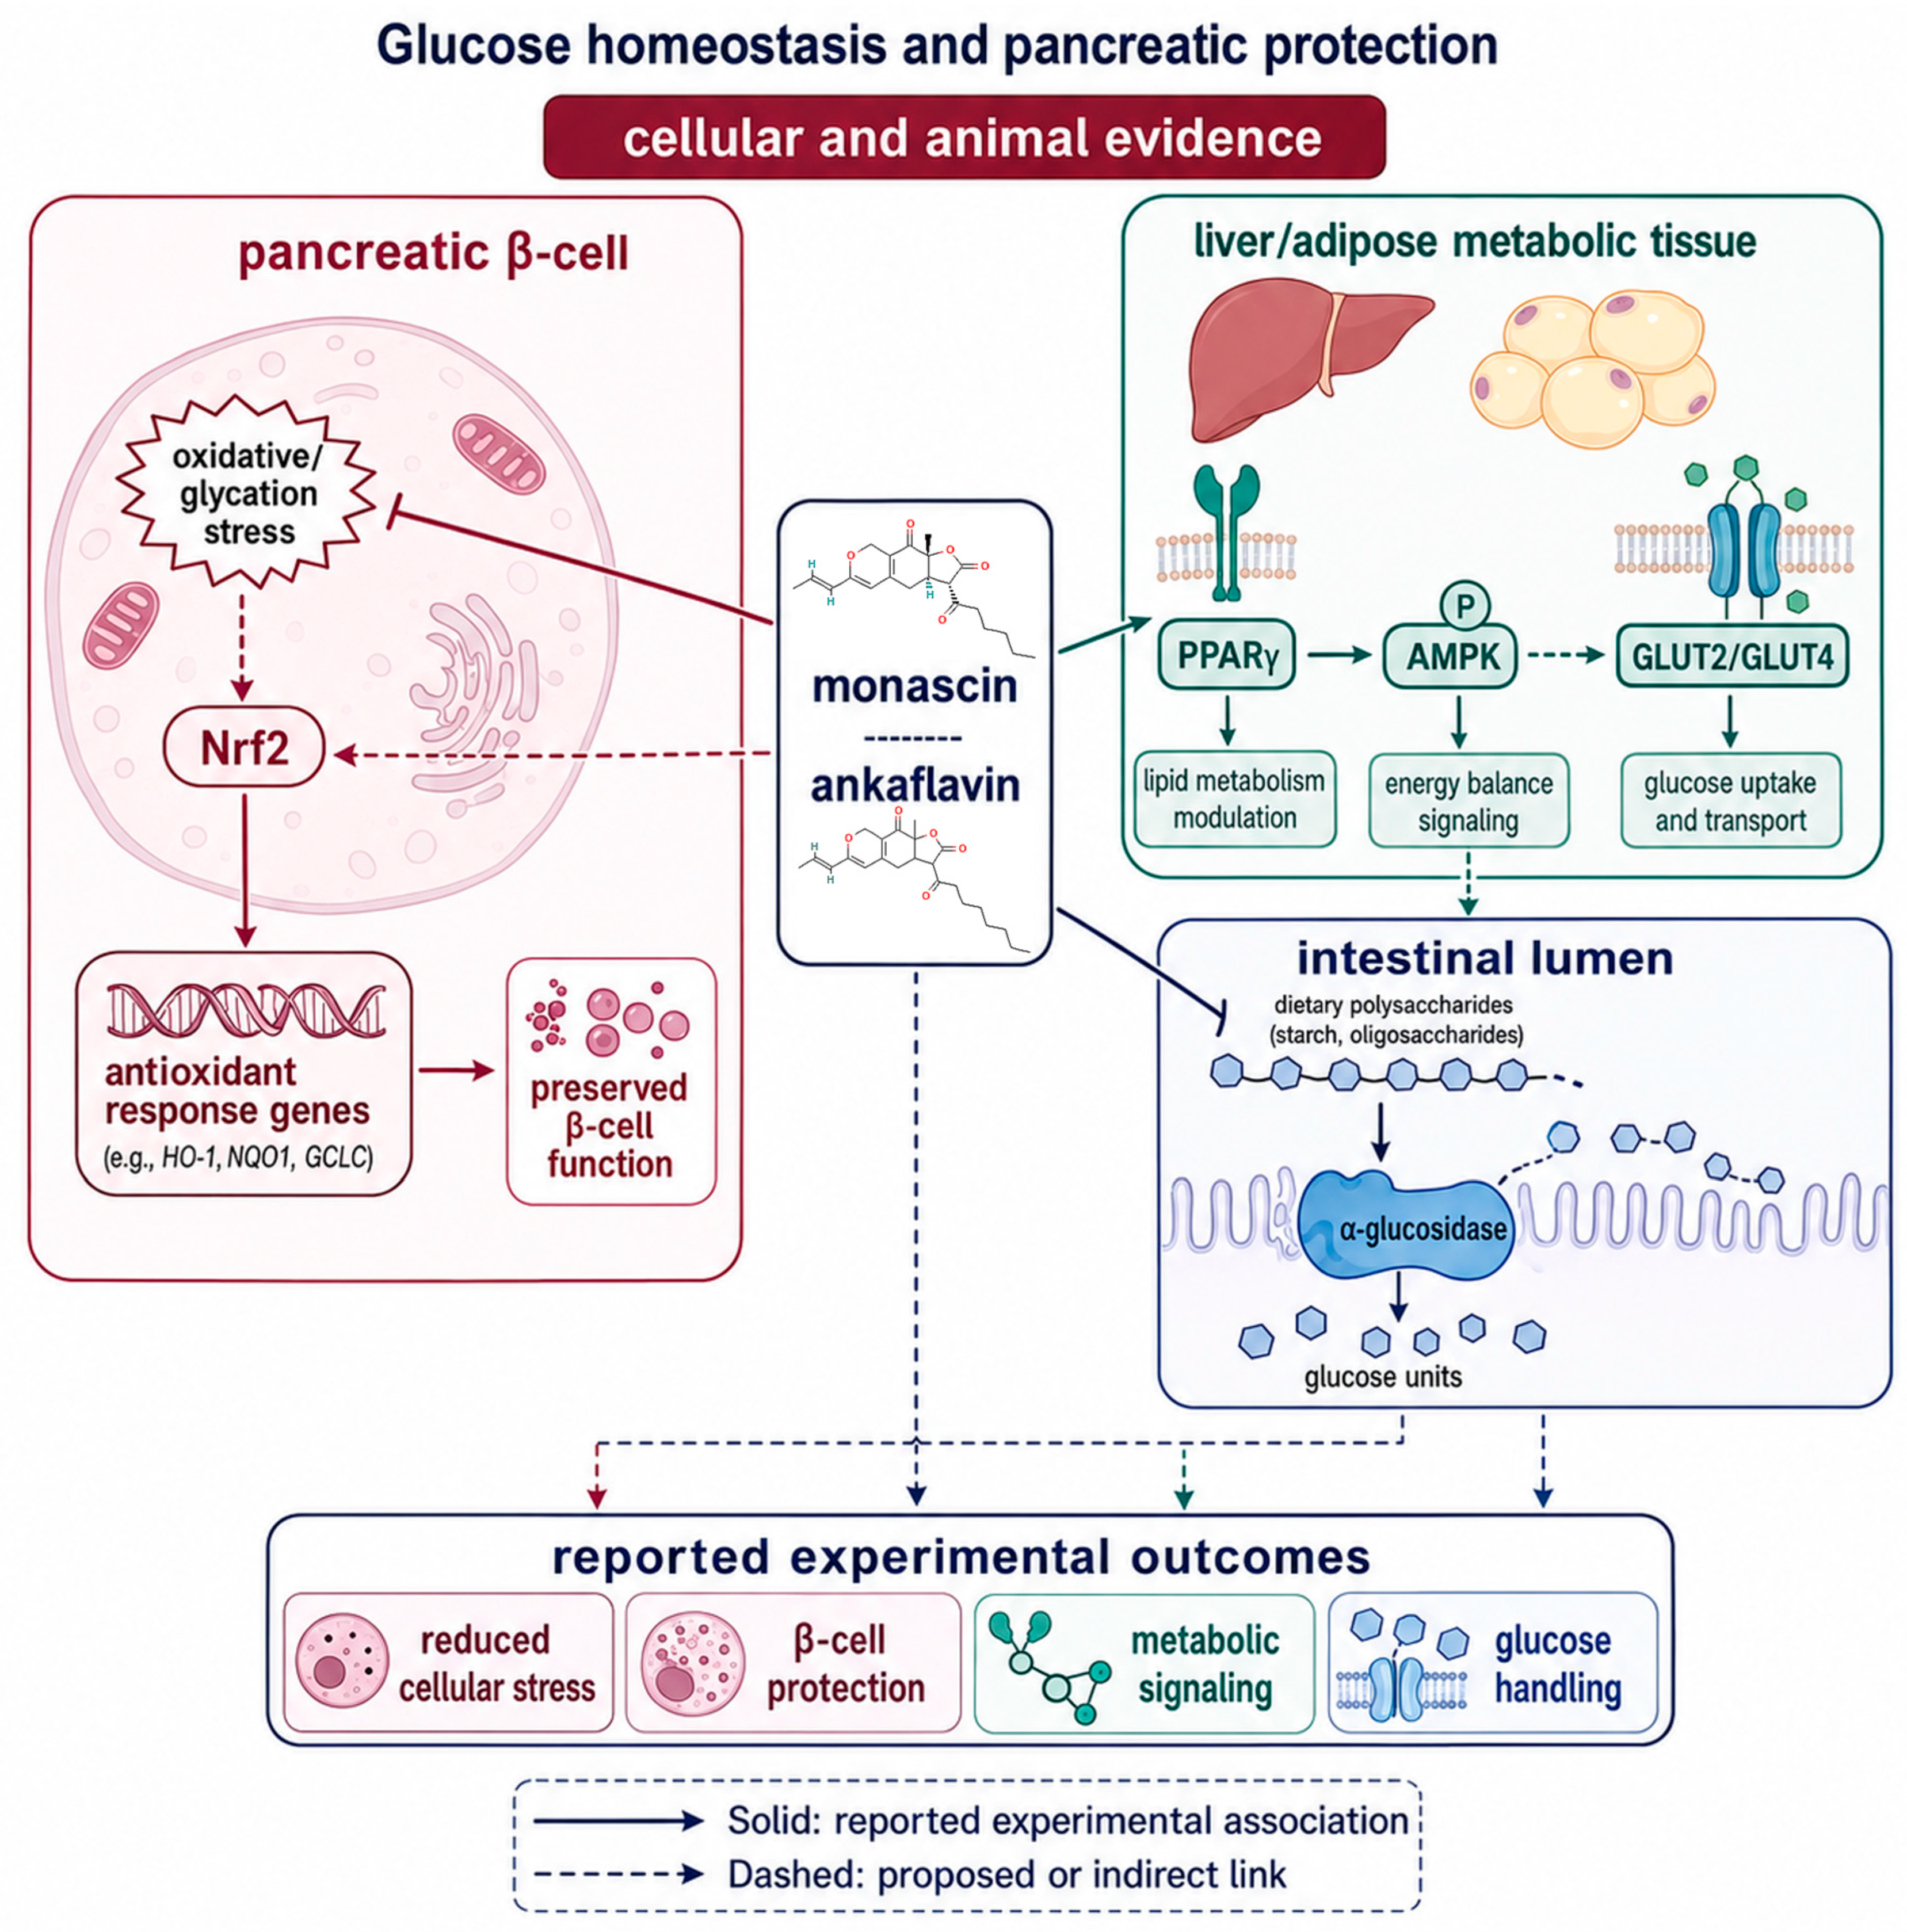
Monascus-derived azaphilone compounds, particularly monascin and ankaflavin, have been investigated for possible effects on glucose-related pathways. Experimental studies have reported α-glucosidase inhibition and anti-glycation activity for these compounds [79]. Other proposed effects on insulin resistance, glucose uptake, and oxidative-stress responses are supported mainly by cellular and animal evidence [14,16]. The available evidence does not establish clinical glucose-control efficacy for isolated pigments.
5.1. Molecular Mechanisms of Ameliorating Insulin Resistance
Experimental evidence suggests that oxidative stress and inflammation may contribute to insulin resistance. Monascin has been reported in cellular models to attenuate methylglyoxal- and hyperglycemia-related toxicity through PPAR-γ- and Nrf2-associated pathways [16]. These mechanistic observations require confirmation in standardized human studies.
5.2. Protective Effects on Pancreatic β-Cells: Evidence from the RINm5F Model
Pancreatic β-cells are susceptible to oxidative stress and advanced glycation end products. This susceptibility provides a rationale for investigating monascin in β-cell-relevant experimental systems; however, the relevance of these observations to pancreatic protection in humans remains uncertain [16].
5.3. Experimental Findings and Limited Human Evidence
Monascus yellow pigments may affect glucose-related pathways through mechanisms such as α-glucosidase inhibition and anti-glycation activity, which have been reported primarily in experimental systems [79]. Cellular and animal findings provide a rationale for continued investigation of glucose-related and oxidative-stress pathways [18,20]. Larger and longer human trials with well-characterized interventions are needed before conclusions about clinical glucose control can be drawn (Figure 4).
Figure 4.
Experimental evidence on glucose-related and oxidative-stress pathways associated with monascin and ankaflavin. Created by the authors based on cellular and animal studies of PPAR-γ-, Nrf2-, α-glucosidase-, and anti-glycation-related outcomes [16,79]. Icons denote the experimental systems and reported mechanistic endpoints summarized in the figure.
6. Cardiovascular Outcomes: Evidence from SHR Models and Limited Human Studies
Cardiovascular diseases (CVDs), including hypertension and atherosclerosis, are associated with endothelial dysfunction and vascular remodeling. Monascus-fermented products have been investigated for cardiovascular-related outcomes, but effects cannot be attributed to individual yellow pigments when complex preparations are used. Experimental studies have examined monascin and ankaflavin in relation to endothelial, inflammatory, and blood-pressure-related pathways; the clinical relevance of these observations remains uncertain and requires confirmation in standardized human trials [80].
6.1. Blood Pressure Control in Spontaneously Hypertensive Rat (SHR) Models
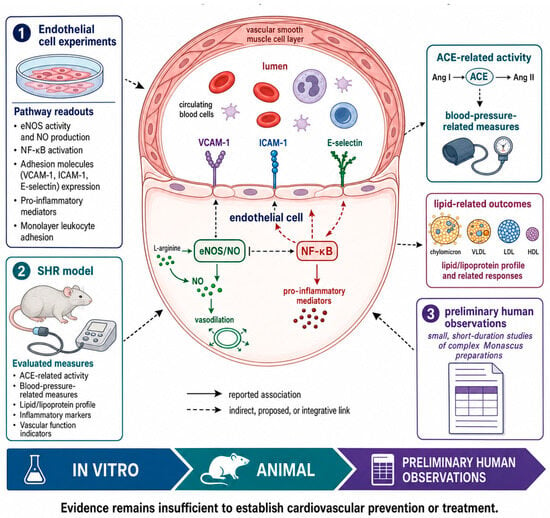
Direct evidence from spontaneously hypertensive rat (SHR) models remains insufficient to attribute blood-pressure control to isolated monascin or ankaflavin. Available reports instead comprise mechanistic, endothelial-cell, and short-term studies of complex Monascus-fermented preparations; therefore, blood-pressure effects should be treated as a research question rather than an established functional claim [4,5,80].
6.2. Vascular Protection and Endothelial Function
Endothelial dysfunction is a major hallmark of cardiovascular disease, characterized by reduced nitric oxide (NO) bioavailability and elevated inflammatory activation. Hsu et al. demonstrated that monascin and ankaflavin exert direct protective effects on human umbilical vein endothelial cells (HUVECs) exposed to tumor necrosis factor-alpha (TNF-α) [80]. These pigments significantly suppress the expression of endothelial adhesion molecules, such as vascular cell adhesion molecule-1 (VCAM-1), intercellular adhesion molecule-1 (ICAM-1), and E-selectin, by inhibiting the phosphorylation of extracellular signal-regulated kinase (ERK) and the nuclear translocation of nuclear factor kappa B (NF-κB). Furthermore, they upregulate endothelial nitric oxide synthase (eNOS) expression, leading to increased NO production which is essential for maintaining vascular tone, inhibiting platelet aggregation, and protecting against endothelial injury [80].
6.3. Limited Human Evidence for Blood-Pressure and Metabolic Outcomes
The translational relevance of cardiovascular findings has only been explored in small studies of complex Monascus-fermented preparations. A randomized, double-blind study of Ankascin 568 plus reported changes in blood-lipid measures over a short intervention period [5]. These observations are preliminary because the intervention was a complex preparation, the study duration was short, and direct comparisons with established lipid-lowering or antihypertensive therapies are lacking.
Cellular and animal studies of Monascus-fermented preparations suggest possible links between monascin- and ankaflavin-containing products and blood-pressure, endothelial, lipid, glucose, and oxidative-stress outcomes (Figure 5) [80]. Small human studies of complex preparations provide preliminary observations, but do not establish clinical safety or efficacy for cardiovascular-disease prevention or management [5]. Future studies should use standardized pigment composition, prespecified safety monitoring, adequate sample sizes, longer follow-up, and appropriate active comparators.
Figure 5.
Reported experimental mechanisms and cardiovascular-related outcomes of Monascus yellow pigments. Created by the authors based on animal, endothelial-cell, and limited human studies of complex Monascus-fermented preparations [5,80].
7. Safety Profile: Comparative Toxicological Analysis Between Yellow Pigments and Monacolin K
Red mold rice contains multiple secondary metabolites, including yellow azaphilone pigments such as monascin and ankaflavin and, in some products, monacolin K. Monacolin K is chemically and pharmacologically identical to lovastatin and therefore has statin-like safety concerns. Monascin- and ankaflavin-rich preparations have shown comparatively low toxicity signals under the tested experimental and short-term clinical conditions, but the available evidence is insufficient to establish an intrinsic safety advantage. Direct, standardized head-to-head toxicological comparisons remain unavailable, and interpretation is complicated by variation in monacolin K, citrinin, pigment composition, dose, and product labeling [66,81].
7.1. Toxicological Concerns Associated with Monacolin K
Monacolin K is the most renowned lipid-lowering component in red mold rice, yet it is also the subject of the greatest safety controversy. Its primary toxicological risks revolve around muscle toxicity, such as myopathy and rhabdomyolysis, and hepatotoxicity. The European Food Safety Authority (EFSA) warned that monacolin K exposure from dietary supplements often falls within the therapeutic dose range of lovastatin [67]. Extensive adverse event data support that an intake of 10 mg/day poses significant safety concerns, and severe adverse reactions have been reported at doses as low as 3 mg/day [67]. Clinical case studies continue to report incidents of fulminant red mold rice-associated rhabdomyolysis, acute liver injury, and hyperkalemia [82,83]. EFSA was unable to establish a daily intake of monacolins from red yeast rice that does not raise health concerns. Commission Regulation (EU) 2022/860 requires an individual portion recommended for daily consumption to provide less than 3 mg of monacolins from red yeast rice and mandates specified label warnings. Furthermore, adverse event reporting systems and available meta-analyses continue to associate red yeast rice extract use with muscle symptoms and liver dysfunction [84]. Animal studies offer biological plausibility for these adverse effects; acute administration of red mold rice significantly depletes coenzyme Q10 (CoQ10) levels in murine liver and heart tissues, a phenomenon perfectly aligning with the statin-induced suppression of the mevalonate pathway [85]. Additionally, research demonstrates that monacolin K exerts an inhibitory effect on cytochrome P450 (CYP450) and P-glycoprotein (P-gp) that is even stronger than pure lovastatin, substantially increasing the risk of drug–drug interactions [86].
Systematic safety analyses and medication-safety reviews likewise emphasize that red yeast rice adverse-event risk cannot be evaluated only by traditional-use history; dose, product quality, and patient susceptibility remain central considerations [87,88].
Clinical and review literature on red yeast rice further supports the need for careful monacolin K standardization, because efficacy in mild dyslipidemia must be balanced against supplement variability and statin-like safety concerns [89,90,91].
7.2. Safety Profile of Yellow Pigments: Monascin and Ankaflavin
Current evidence suggests that monascin- and ankaflavin-rich preparations may have a different short-term safety profile from monacolin K-containing products. In a 12-week double-blind study of Ankascin 568 plus, no significant abnormalities in measured liver, kidney, thyroid, electrolyte, or CPK indices were reported [5]. These findings should not be interpreted as proof of comprehensive safety: the human evidence is limited in size and duration, and hepatic, renal, gastrointestinal, metabolic, reproductive, drug-interaction, and long-term outcomes require systematic assessment. Results obtained from a fermented extract cannot be assumed to apply to isolated yellow pigments or to all commercial products.
7.3. Comparative Toxicological Interpretation and Quality Control
The safety interpretation of Monascus yellow pigments and monacolin K should be based on the nature and level of available evidence rather than on an assumed intrinsic safety hierarchy (Table 5). Monacolin K is chemically identical to lovastatin and is therefore associated with statin-like adverse-effect and interaction concerns; however, the risk in red mold rice products also depends on dose, product composition, and quality control. For monascin and ankaflavin, the available evidence is mainly mechanistic, animal, and short-term human research on complex fermented preparations. For monascinol, the evidence is currently preclinical. Consequently, direct claims of superior efficacy or comprehensive safety are not supported by standardized head-to-head clinical trials. Citrinin control, compositional standardization, chronic toxicology, pharmacokinetics, and interactions with medicines remain essential considerations for all Monascus-derived products [66,67,68,81,92,93].
Table 5.
Comparative overview of reported efficacy, safety, mechanisms, and evidence levels for major Monascus yellow pigments and monacolin K.
8. Future Research: Monascinol and Gut-Microbiota-Related Outcomes
8.1. Discovery and Preclinical Evidence for Monascinol
As research into Monascus-fermented products progresses beyond traditional red pigments and monacolin K, monascinol has emerged as a yellow azaphilone of interest. Studies of Monascus pilosus SWM-008-fermented red mold rice have reported associations between its functional components, gut-microbiota changes, and metabolic outcomes in rats [94]. These observations are preclinical and should not be interpreted as evidence of biological superiority or established safety in humans. Monascinol is therefore a candidate for further functional-food research rather than a clinically validated alternative to monacolin K.
8.2. Reported Associations with Gut Microbiota Composition
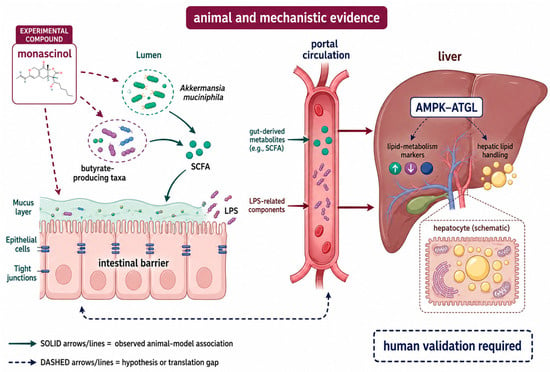
The reported microbiota-related effects of monascinol are currently based on animal studies. In normal- and high-fat-diet models, Monascus pilosus SWM-008-fermented red mold rice and its functional components were associated with changes in the relative abundance of taxa including Akkermansia muciniphila, Ligilactobacillus murinus, and Duncaniella dubosii [94]. These findings do not establish causality, clinical benefit, or safety in humans; they should be interpreted as hypothesis-generating observations requiring confirmation by targeted metabolomics, functional studies, and human trials.
8.3. Akkermansia muciniphila and Short-Chain-Fatty-Acid-Related Findings
Akkermansia muciniphila is a health-associated bacterium of interest in metabolic and intestinal research, but its relevance to monascinol remains preclinical [95]. Other Monascus-pigment studies have reported gut-level effects in disease models [96,97]. Accordingly, microbiota-related observations should not be interpreted as evidence of clinical benefit or as a regulatory classification of monascinol.
8.4. Mechanisms of Metabolic Regulation: The Gut–Liver Axis and Lipid Oxidation
Current animal studies suggest that microbiota-associated changes may coexist with metabolic outcomes, but they do not establish a causal gut–liver-axis mechanism or a specific effect on lipid oxidation for monascinol. Such mechanisms should be tested with standardized preparations, targeted metabolomics, tissue-level pathway analyses, and intervention studies designed to distinguish direct compound effects from changes in the food matrix or microbiota [94,96,97,98].
8.5. Experimental Organ-Related Outcomes and Research Directions
In experimental hyperuricemia models, monascin and ankaflavin have been reported to affect two relevant mechanisms, competitively binding to the active site of xanthine oxidase (XOD) to inhibit uric acid production, while concurrently modulating the expression of uric acid transporters to facilitate excretion [98].
8.6. Safety Profile and Future Research Perspectives
The available safety observations for monascinol are preclinical. An eight-week rat study of Monascus pilosus SWM-008-fermented red mold rice and its functional components reported no significant adverse changes in body weight or selected hepatic and renal biomarkers [94]. This cannot be considered clinical evidence or sufficient long-term toxicological evaluation. Future work should include standardized material characterization, dose-ranging and chronic-toxicity studies, pharmacokinetics, interaction assessments, and adequately powered randomized controlled trials in humans. Until such evidence is available, descriptions of monascinol as a postbiotic-like ingredient should remain exploratory (Figure 6).
Figure 6.
Schematic overview of reported monascinol-associated outcomes in gut microbiota, metabolic regulation, and organ-related experimental models. Created by the authors based on animal and mechanistic studies of SWM-008 fermented rice, monascinol, and gut microbiota [94].
9. Conclusion: Research Priorities for Monascus Yellow Pigments as Functional-Food Ingredients
9.1. From Traditional Colorants to Candidate Functional Ingredients
Monascus species have long been used in Asian food and medicinal applications, traditionally as sources of colorants and fermentation-derived metabolites [1]. Yellow pigments such as monascin and ankaflavin, together with the derivative monascinol, are now being investigated for their physicochemical properties and biological activities. Although experimental studies suggest potential advantages for selected applications, current evidence does not establish superior efficacy, comprehensive safety, or broad clinical utility relative to traditional ingredients or established therapies. Development should therefore proceed through standardized composition, matrix-specific stability and bioavailability testing, contaminant control, chronic safety assessment, and adequately powered human trials [4,8].
9.2. Reported Metabolic Mechanisms and Safety Evidence Gaps
Monascus yellow pigments are of interest for next-generation functional foods because experimental studies suggest multi-target activity under tested conditions. Monascin and ankaflavin have been reported to interact with PPAR-α/PPAR-γ- and AMPK-associated pathways [14,15], and experimental studies have described effects relevant to lipid metabolism, glucose homeostasis, endothelial function, and oxidative stress [5,14,15]. These mechanistic and preclinical data should not be equated with efficacy comparable to monacolin K or with a proven absence of statin-associated adverse effects. Their potential value as functional ingredients should therefore be assessed through standardized composition, bioavailability, dose–response, long-term safety, and human-efficacy studies [67,68].
9.3. Gut Microbiota Findings and Requirements for Human Validation
Monascinol has generated interest because animal studies of Monascus pilosus SWM-008-fermented red mold rice have reported associations with gut-microbiota changes and metabolic phenotypes [94]. These data are preclinical, and the causal contribution of microbiota changes has not been established in humans. Monascinol may be a useful research lead for precision nutrition, but its safety, bioavailability, dose, regulatory status, and clinical relevance remain to be determined.
9.4. Process Optimization and Development Prospects for Functional Foods
To meet growing market demand, large-scale production technologies for Monascus yellow pigments are continuously advancing. Precision-fermentation approaches, including supplementation with specific nitrogen sources and calcium chloride, can redirect metabolic flux toward yellow pigment synthesis [11,62]. Additional process strategies, including dual mutagenesis, CRISPR-based strain engineering, and low-cost substrate use, further support scalable pigment production [63,64,65].
9.5. Food-Matrix Stability, Bioavailability, and Application Perspectives
Potential food applications should be considered in relation to the final food matrix rather than only to pigment yield. Light, heat, oxygen, pH, water activity, and interactions with proteins, lipids, carbohydrates, and minerals may alter pigment stability, color expression, and bioaccessibility. Encapsulation and delivery-system studies suggest possible strategies for protecting Monascus pigments, but performance must be evaluated in the intended food matrix and cannot be assumed from model systems [8,9,10].
Appropriate application concepts may include fermented cereal-based foods, beverages, dairy- or plant-based matrices, and lipid-containing foods where sensory acceptance, dose delivery, and stability can be jointly assessed. Any health-oriented application should specify the pigment composition, serving dose, co-occurring monacolin K and citrinin levels, and storage conditions. Human outcomes should not be inferred from antioxidant capacity, in vitro bioaccessibility, or animal studies alone [8,9,10,28,68].
Future studies should compare stability and bioavailability across representative matrices, assess interactions with food components, and evaluate whether processing changes the chemical profile. This matrix-specific evidence, together with standardized manufacturing and safety data, is necessary before health claims or broad functional-food positioning can be supported [8,9,10,28,68].
In summary, monascin, ankaflavin, and monascinol are Monascus yellow pigments with mechanistic and preclinical evidence relevant to lipid and glucose metabolism, vascular biology, and gut-microbiota-associated outcomes. Small, short-duration studies of selected Monascus-fermented preparations provide preliminary human observations, but do not establish the long-term efficacy or safety of individual pigments. Future research should prioritize standardized composition and dose, contaminant control, pharmacokinetics and food-matrix effects, chronic safety evaluation, and adequately powered randomized controlled trials. On the basis of the current evidence, Monascus yellow pigments should be considered promising candidate functional ingredients for further evaluation rather than established interventions for metabolic syndrome (Figure 7) [4,99].
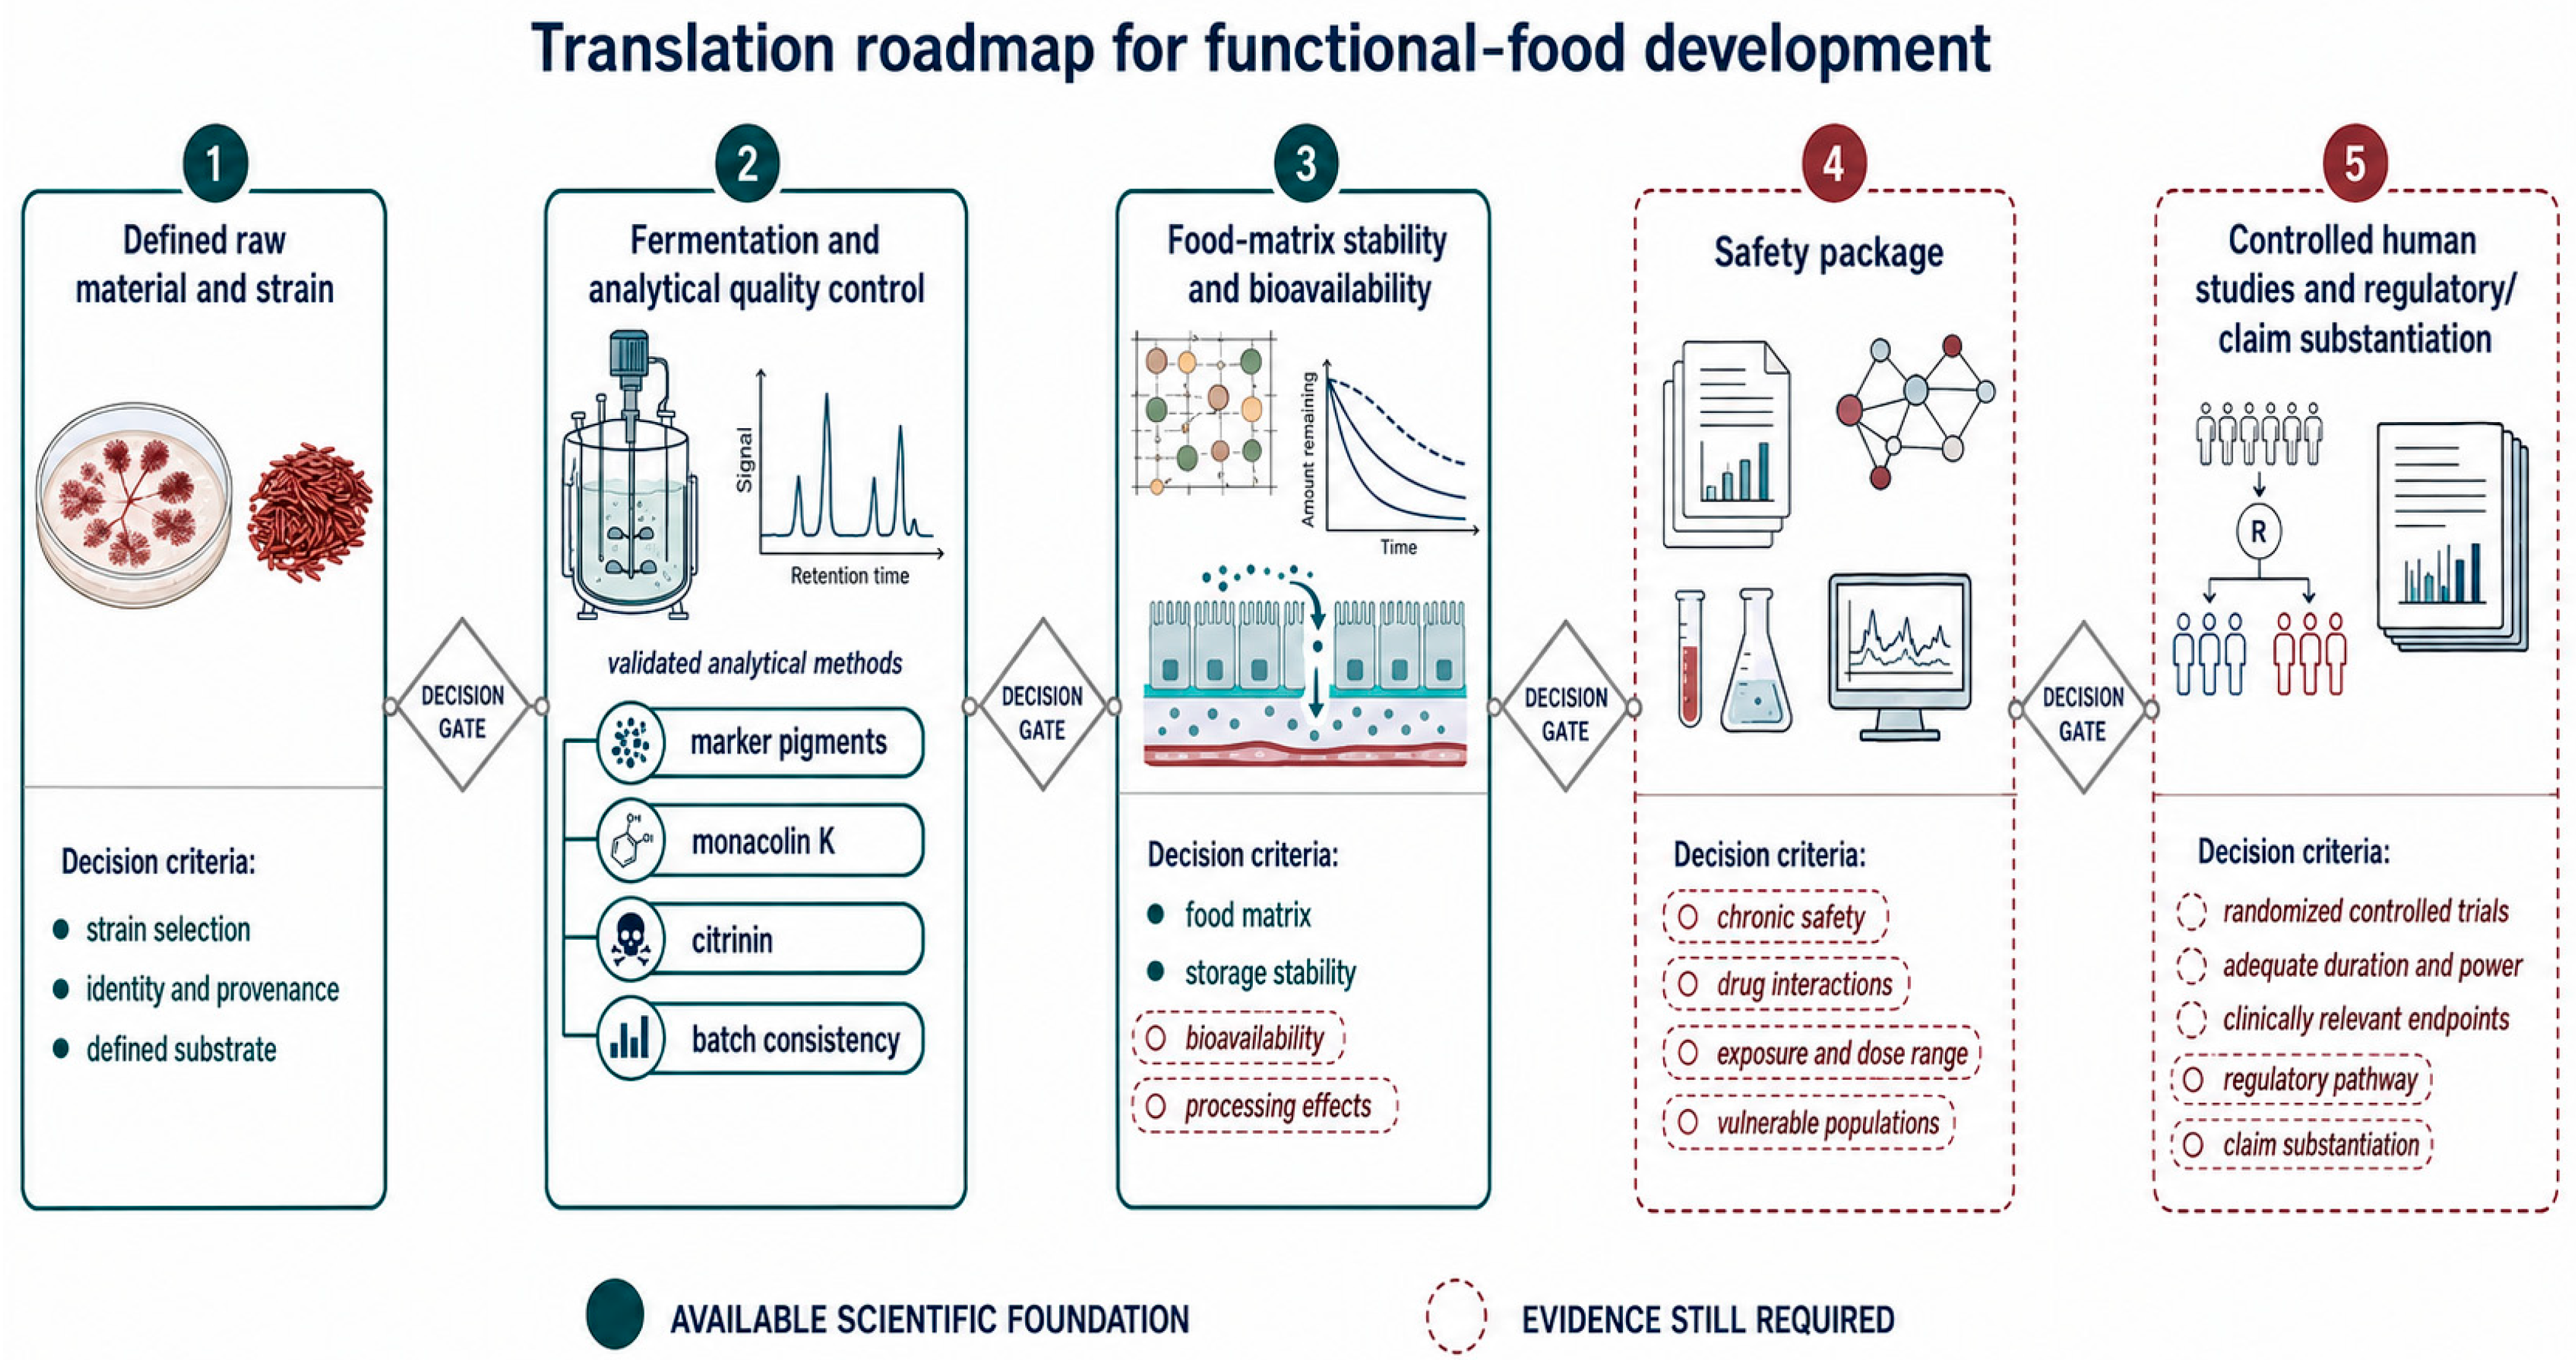
Figure 7.
Integrated overview of the reported biological evidence and future research priorities for Monascus yellow pigments. This framework summarizes the evidence and research gaps reviewed in this article, including quality control, safety, production, and translational requirements [28,68,99].
Author Contributions
Conceptualization, C.-L.L. and T.-M.P.; writing—original draft preparation, C.-L.L.; writing—review and editing, C.-L.L. and T.-M.P.; supervision, T.-M.P. All authors have read and agreed to the published version of the manuscript.
Funding
This research received no external funding.
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
No new data were created or analyzed in this study. Data sharing is not applicable to this article.
Conflicts of Interest
Tzu-Ming Pan is the Chief Technology Officer of SunWay Biotech Co., Taipei, Taiwan. This affiliation did not influence the design, analysis, interpretation, or reporting of this review. The authors declare no conflicts of interest relevant to this review.
References
- Hong, X.; Deng, J.; Liu, J.; Zhong, H.; Ren, J.; Zhou, B. Research advances in yellow pigments derived from Monascus, an edible filamentous fungus. Adv. Appl. Microbiol. 2025, 132, 83–122. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Patakova, P. Monascus secondary metabolites: Production and biological activity. J. Ind. Microbiol. Biotechnol. 2013, 40, 169–181. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Feng, Y.; Shao, Y.; Chen, F. Monascus pigments. Appl. Microbiol. Biotechnol. 2012, 96, 1421–1440. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lin, C.H.; Lin, T.H.; Pan, T.M. Alleviation of metabolic syndrome by monascin and ankaflavin: The perspective of Monascus functional foods. Food Funct. 2017, 8, 2102–2109. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, S.F.; Wang, Y.R.; Shen, Y.C.; Chen, C.L.; Huang, C.N.; Pan, T.M.; Wang, C.K. A randomized, double-blind clinical study of the effects of Ankascin 568 plus on blood lipid regulation. J. Food Drug Anal. 2018, 26, 393–400. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Adin, S.N.; Gupta, I.; Panda, B.P.; Mujeeb, M. Monascin and ankaflavin-Biosynthesis from Monascus purpureus, production methods, pharmacological properties: A review. Biotechnol. Appl. Biochem. 2023, 70, 137–147. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- He, J.; Jia, M.; Li, W.; Deng, J.; Ren, J.; Luo, F.; Bai, J.; Liu, J. Toward improvements for enhancement the productivity and color value of Monascus pigments: A critical review with recent updates. Crit. Rev. Food Sci. Nutr. 2022, 62, 7139–7153. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, G.; Wu, Z. Production and biological activities of yellow pigments from Monascus fungi. World J. Microbiol. Biotechnol. 2016, 32, 160. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Vendruscolo, F.; Meinicke Bühler, R.M.; Cesar de Carvalho, J.; de Oliveira, D.; Moritz, D.E.; Schmidell, W.; Ninow, J.L. Monascus: A Reality on the Production and Application of Microbial Pigments. Appl. Biochem. Biotechnol. 2016, 178, 211–223. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dudek, A.; Pietrzak, M.; Benkowska-Biernacka, D.; Pruchnik, H.; Boratynski, F.; El-Sayed, E.R. Nanoliposomal Encapsulation of Red, Yellow, and Orange Natural Pigments from Monascus ruber: Characterization, Stability, and Biological Activities. Curr. Microbiol. 2025, 82, 259. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bai, Y.; Zhang, W.; Guo, R.; Yu, J.; Wang, Y. Enhancement of yellow pigments production via high CaCl2 stress fermentation of Monascus purpureus. FEMS Microbiol. Lett. 2024, 371, fnae012. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, H.; Zhang, J.; Lu, G.; Wang, F.; Shu, L.; Xu, H.; Li, Z.; Wang, Y.; Guo, Q.; Wu, S.; et al. Comparative metabolomics analysis reveals the metabolic regulation mechanism of yellow pigment overproduction by Monascus using ammonium chloride as a nitrogen source. Appl. Microbiol. Biotechnol. 2021, 105, 6369–6379. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, C.; Sun, Q.; Yang, L.; Ablimit, A.; Dong, H.; Wang, H.; Wang, C.; Wang, C. Mutation breeding of Monascus to produce a high yield of orange pigment and low citrinin content using the ARTP method. J. Fungi 2024, 10, 553. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hsu, W.H.; Chen, T.H.; Lee, B.H.; Hsu, Y.W.; Pan, T.M. Monascin and ankaflavin act as natural AMPK activators with PPARα agonist activity to down-regulate nonalcoholic steatohepatitis in high-fat diet-fed C57BL/6 mice. Food Chem. Toxicol. 2014, 64, 94–103. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lee, C.L.; Wen, J.Y.; Hsu, Y.W.; Pan, T.M. Monascus-fermented yellow pigments monascin and ankaflavin showed antiobesity effect via the suppression of differentiation and lipogenesis in obese rats fed a high-fat diet. J. Agric. Food Chem. 2013, 61, 1493–1500. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hsu, W.H.; Lee, B.H.; Chang, Y.Y.; Hsu, Y.W.; Pan, T.M. A novel natural Nrf2 activator with PPARγ-agonist (monascin) attenuates the toxicity of methylglyoxal and hyperglycemia. Toxicol. Appl. Pharmacol. 2013, 272, 842–851. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tan, H.; Xing, Z.; Chen, G.; Tian, X.; Wu, Z. Evaluating antitumor and antioxidant activities of yellow Monascus pigments from Monascus ruber fermentation. Molecules 2018, 23, 3242. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, L.; Zhao, J.; Huang, Y.; Xin, Q.; Wang, Z. Diversifying of Chemical Structure of Native Monascus Pigments. Front. Microbiol. 2018, 9, 3143. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cheng, M.J.; Wu, M.D.; Chen, I.S.; Chen, C.Y.; Lo, W.L.; Yuan, G.F. Secondary metabolites from the red mould rice of Monascus purpureus BCRC 38113. Nat. Prod. Res. 2010, 24, 1719–1725. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cheng, M.J.; Wu, M.D.; Chen, I.S.; Yuan, G.F. A new sesquiterpene isolated from the extracts of the fungus Monascus pilosus-fermented rice. Nat. Prod. Res. 2010, 24, 750–758. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, S.; Su, D.X.; Gao, M.X.; Zhang, J.L.; Liu, Y.B.; Wu, Q.H.; Yang, H.L.; Li, L. A facile macroporous resin-based method for separation of yellow and orange Monascus pigments. Food Sci. Biotechnol. 2021, 30, 545–553. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yang, H.; Li, J.; Wang, Y.; Gan, C. Identification of water-soluble Monascus yellow pigments using HPLC-PAD-ELSD, high-resolution ESI-MS, and MS-MS. Food Chem. 2018, 245, 536–541. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xu, J.Y.; Li, H.Q.; Chen, J.M.; Chen, F.Z. Crystal structure and characterization of monascin from the extracts of Monascus purpureus-fermented rice. Acta Crystallogr. Sect. C 2024, 80, 425–433. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Su, N.W.; Lin, Y.L.; Lee, M.H.; Ho, C.Y. Ankaflavin from Monascus-fermented red rice exhibits selective cytotoxic effect and induces cell death on Hep G2 cells. J. Agric. Food Chem. 2005, 53, 1949–1954. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jongrungruangchok, S.; Kittakoop, P.; Yongsmith, B.; Bavovada, R.; Tanasupawat, S.; Lartpornmatulee, N.; Thebtaranonth, Y. Azaphilone pigments from a yellow mutant of the fungus Monascus kaoliang. Phytochemistry 2004, 65, 2569–2575. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Husakova, M.; Patakova, P. Purified Monascus pigments: Biological activities and mechanisms of action. J. Nat. Prod. 2025, 88, 607–615. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lee, C.L.; Kung, Y.H.; Wu, C.L.; Hsu, Y.W.; Pan, T.M. Monascin and ankaflavin act as novel hypolipidemic and high-density lipoprotein cholesterol-raising agents in red mold dioscorea. J. Agric. Food Chem. 2010, 58, 9013–9019. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Farawahida, A.H.; Palmer, J.; Flint, S. Monascus spp. and citrinin: Identification, selection of Monascus spp. isolates, occurrence, detection and reduction of citrinin during the fermentation of red fermented rice. Int. J. Food Microbiol. 2022, 379, 109829. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, Q.; Zhong, S.; Wang, X.; Gao, S.; Yang, X.L.; Chen, F.; Molnár, I. An integrated approach to determine the boundaries of the azaphilone pigment biosynthetic gene cluster of Monascus ruber M7 grown on potato dextrose agar. Front. Microbiol. 2021, 12, 744421. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Duan, Y.; Ma, H.; Wei, X.; Li, M. Dynamic regulation of Monascus azaphilones biosynthesis by the binary MrPigE-MrPigF oxidoreductase system. Appl. Microbiol. Biotechnol. 2022, 106, 7519–7530. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, J.; Yang, S.; Wang, Q.; Liu, Q.; Chen, J.; Gong, Y.; Xu, R.; Shao, Y. Enhancement of Monascus azaphilone pigments production without citrinin contamination by targeting overexpression of histone acetyltransferase MrEsa1 and deletion of polyketide synthase PksCT. J. Fungi 2026, 12, 126. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Balakrishnan, B.; Kim, H.J.; Suh, J.W.; Chen, C.C.; Liu, K.H.; Park, S.; Kwon, H. Monascus azaphilone pigment biosynthesis employs a dedicated fatty acid synthase for short chain fatty acyl moieties. J. Korean Soc. Appl. Biol. Chem. 2014, 57, 191–196. [Google Scholar] [CrossRef] [Scilit]
- Chen, W.; Feng, Y.; Molnár, I.; Chen, F. Nature and nurture: Confluence of pathway determinism with metabolic and chemical serendipity diversifies Monascus azaphilone pigments. Nat. Prod. Rep. 2019, 36, 561–572. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhen, Z.; Xiong, X.; Liu, Y.; Zhang, J.; Wang, S.; Li, L.; Gao, M. NaCl Inhibits Citrinin and Stimulates Monascus Pigments and Monacolin K Production. Toxins 2019, 11, 118. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, L.; Chen, S.; Gao, M.; Ding, B.; Zhang, J.; Zhou, Y.; Liu, Y.; Yang, H.; Wu, Q.; Chen, F. Acidic conditions induce the accumulation of orange Monascus pigments during liquid-state fermentation of Monascus ruber M7. Appl. Microbiol. Biotechnol. 2019, 103, 8393–8402. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Balakrishnan, B.; Park, S.; Kwon, H. Inactivation of the oxidase gene mppG results in the selective loss of orange azaphilone pigments in Monascus purpureus. Appl. Biol. Chem. 2017, 60, 437–446. [Google Scholar] [CrossRef] [Scilit]
- Pavesi, C.; Flon, V.; Mann, S.; Leleu, S.; Prado, S.; Franck, X. Biosynthesis of azaphilones: A review. Nat. Prod. Rep. 2021, 38, 1058–1071. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Meng, Z.; Tan, Y.; Duan, Y.; Li, M. Metabolic modulation of TCA cycle by S-nitrosylation in Monascus spp. Synth. Syst. Biotechnol. 2026, 12, 490–501. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nie, M.; Liu, T.; Qiu, X.; Yang, J.; Liu, J.; Ren, J.; Zhou, B. Regulation mechanism of lipids for extracellular yellow pigments production by Monascus purpureus BWY-5. Appl. Microbiol. Biotechnol. 2023, 107, 5191–5208. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, J.; Du, Y.; Ma, H.; Pei, X.; Li, M. Enhancement of Monascus yellow pigments production by activating the cAMP signalling pathway in Monascus purpureus HJ11. Microb. Cell Fact. 2020, 19, 224. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wan, R.; Wang, Z.; Li, Y.; Zeng, X.; Xin, B.; Qiao, J.; Zeng, H.; Zhang, L. Mechanistic insights into isopropyl myristate-stimulated Monascus pigment biosynthesis via untargeted metabolomics. World J. Microbiol. Biotechnol. 2026, 42, 24. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xiong, X.; Zhang, X.; Wu, Z.; Wang, Z. Accumulation of yellow Monascus pigments by extractive fermentation in nonionic surfactant micelle aqueous solution. Appl. Microbiol. Biotechnol. 2015, 99, 1173–1180. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lv, J.; Zhang, B.B.; Liu, X.D.; Zhang, C.; Chen, L.; Xu, G.R.; Cheung, P.C.K. Enhanced production of natural yellow pigments from Monascus purpureus by liquid culture: The relationship between fermentation conditions and mycelial morphology. J. Biosci. Bioeng. 2017, 124, 452–458. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, M.; Huang, T.; Chen, G.; Wu, Z. Production of water-soluble yellow pigments via high glucose stress fermentation of Monascus ruber CGMCC 10910. Appl. Microbiol. Biotechnol. 2017, 101, 3121–3130. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lv, J.; Qian, G.F.; Chen, L.; Liu, H.; Xu, H.X.; Xu, G.R.; Zhang, B.B.; Zhang, C. Efficient Biosynthesis of Natural Yellow Pigments by Monascus purpureus in a Novel Integrated Fermentation System. J. Agric. Food Chem. 2018, 66, 918–925. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kuang, L.; Ma, P.; He, X.; Wang, L.; Xie, Q.; He, Y.; Tan, H. Effects of VeA gene on the growth, pigment and citrinin synthesis of Monascus ruber M7. Microorganisms 2026, 14, 137. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liang, B.; Du, X.J.; Li, P.; Sun, C.C.; Wang, S. Investigation of Citrinin and Pigment Biosynthesis Mechanisms in Monascus purpureus by Transcriptomic Analysis. Front. Microbiol. 2018, 9, 1374. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, C.; Wang, H.; Sun, Q.; Ablimit, A.; Dong, H.; Wang, C.; Zhai, D.; Zhang, B.; Hu, W.; Liu, C.; et al. Improvement of Monacolin K and pigment production in Monascus by 5-azacytidine. J. Fungi 2024, 10, 819. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, A.; Juan Chen, A.; Liu, B.; Wei, Q.; Bai, J.; Hu, Y. Investigation of citrinin and monacolin K gene clusters variation among pigment producer Monascus species. Fungal Genet. Biol. 2022, 160, 103687. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Feng, S.; Liu, M.; Wang, X.; Wang, L.; Li, T.; Sun, C.; Han, R.; Liang, B. Functional characterization of mpdh as a key dehydratase in citrinin biosynthesis in M. purpureus YY-1. Food Chem. 2026, 502, 148489. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, R.Y.; Zhang, C.Y.; Xiao, S.; Liu, X.Y.; Li, R.X.; Li, J.; Li, H.; Liu, J. Exploring the multifaceted roles of histone deacetylase inhibitor vorinostat in the cell growth, mycelial morphology, pigments, and citrinin biosynthesis of Monascus purpureus. Arch. Microbiol. 2025, 207, 95. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Guo, X.; Li, Y.; Zhang, R.; Yu, J.; Ma, X.; Chen, M.; Wang, Y. Transcriptional regulation contributes more to Monascus pigments diversity in different strains than to DNA sequence variation. World J. Microbiol. Biotechnol. 2019, 35, 138. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, Y.; Wang, N.; Jiao, X.; Tu, Z.; He, Q.; Fu, J. The ctnF gene is involved in citrinin and pigment synthesis in Monascus aurantiacus. J. Basic Microbiol. 2020, 60, 873–881. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, X.; Chen, W.; Wang, C. Regulation of citrinin biosynthesis in Monascus purpureus: Impacts on growth, morphology, and pigments production. Food Microbiol. 2025, 127, 104698. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xiong, L.Q.; Li, Y.Z.; Liang, S.P.; Zhang, C.; Hu, W.L.; Yang, Q.Q.; Molnár, I.; Zhang, B.B. Efficient production of natural yellow azaphilone pigments from Monascus purpureus regulated by microparticle-triggered stress. J. Agric. Food Chem. 2025, 73, 21947–21958. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Huang, J.; Guan, H.W.; Huang, Y.Y.; Lai, K.S.; Chen, H.Y.; Xue, H.; Zhang, B.B. Evaluating the effects of microparticle addition on mycelial morphology, natural yellow pigments productivity, and key genes regulation in submerged fermentation of Monascus purpureus. Biotechnol. Bioeng. 2021, 118, 2503–2513. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yang, S.Z.; Huang, Z.F.; Liu, H.Q.; Hu, X.; Wu, Z.Q. Improving mycelial morphology and adherent growth as well as metabolism of Monascus yellow pigments using nitrate resources. Appl. Microbiol. Biotechnol. 2020, 104, 9607–9617. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Huang, T.; Tan, H.; Chen, G.; Wang, L.; Wu, Z. Rising temperature stimulates the biosynthesis of water-soluble fluorescent yellow pigments and gene expression in Monascus ruber CGMCC10910. AMB Express 2017, 7, 134. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Huang, Z.F.; Yang, S.Z.; Liu, H.Q.; Tian, X.F.; Wu, Z.Q. Sodium starch octenyl succinate facilitated the production of water-soluble yellow pigments in Monascus ruber fermentation. Appl. Microbiol. Biotechnol. 2021, 105, 6691–6706. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Huang, Z.; Hu, T.; Yang, S.; Tian, X.; Wu, Z. Genetic responses to adding nitrates to improve hydrophilic yellow pigment in Monascus fermentation. Appl. Microbiol. Biotechnol. 2023, 107, 1341–1359. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Patrovsky, M.; Sinovska, K.; Branska, B.; Patakova, P. Effect of initial pH, different nitrogen sources, and cultivation time on the production of yellow or orange Monascus purpureus pigments and the mycotoxin citrinin. Food Sci. Nutr. 2019, 7, 3494–3500. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jiang, X.; Qiu, X.; Yang, J.; Zhang, S.; Liu, J.; Ren, J.; Lu, D.; Zhou, X.; Zhou, B. A mutant of Monascus purpureus obtained by carbon ion beam irradiation yielded yellow pigments using various nitrogen sources. Enzym. Microb. Technol. 2023, 162, 110121. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bai, J.; Gong, Z.; Shu, M.; Zhao, H.; Ye, F.; Tang, C.; Zhang, S.; Zhou, B.; Lu, D.; Zhou, X.; et al. Increased Water-Soluble Yellow Monascus Pigment Productivity via Dual Mutagenesis and Submerged Repeated-Batch Fermentation of Monascus purpureus. Front. Microbiol. 2022, 13, 914828. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yoon, H.R.; Han, S.; Shin, S.C.; Yeom, S.C.; Kim, H.J. Improved natural food colorant production in the filamentous fungus Monascus ruber using CRISPR-based engineering. Food Res. Int. 2023, 167, 112651. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, X.; Yan, J.; Chen, J.; Gui, R.; Wu, Y.; Li, N. Potato pomace: An efficient resource for Monascus pigments production through solid-state fermentation. J. Biosci. Bioeng. 2021, 132, 167–173. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Farkouh, A.; Baumgartel, C. Mini-review: Medication safety of red yeast rice products. Int. J. Gen. Med. 2019, 12, 167–171. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Younes, M.; Aggett, P.; Aguilar, F.; Crebelli, R.; Dusemund, B.; Filipic, M.; Frutos, M.J.; Galtier, P.; Gott, D.; Gundert-Remy, U.; et al. EFSA Panel on Food Additives and Nutrient Sources added to Food (ANS), Scientific opinion on the safety of monacolins in red yeast rice. EFSA J. 2018, 16, e05368. [Google Scholar] [PubMed]
- Ma, Y.; Gao, H.M.; Zhang, Y.B.; Li, L.Y.; Liu, X.Q.; Wang, Z.M. Suggestions for revision of quality standards of red yeast rice for medicinal and edible purposes in China. China J. Chin. Mater. Medica 2024, 49, 5659–5673. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xiong, F.; Wei, J.; Zhou, Y.; Shao, Y.; Liu, J.; Chen, F. Exploring the subcellular localization of Monascus pigments biosynthases: Preliminary unraveling of the compartmentalization mechanism. J. Fungi 2024, 10, 375. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, X.; Zhao, H.; Ding, C.; Ding, W.; Guo, Q.; Wang, C. Cell wall remodeling and pH stress coordinately regulate Monascus pigment biosynthesis through transcriptional reprogramming. Foods 2025, 14, 3602. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, W.; Chen, R.; Liu, Q.; He, Y.; He, K.; Ding, X.; Kang, L.; Guo, X.; Xie, N.; Zhou, Y.; et al. Orange, red, yellow: Biosynthesis of azaphilone pigments in Monascus fungi. Chem. Sci. 2017, 8, 4917–4925. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhou, W.; Guo, R.; Guo, W.; Hong, J.; Li, L.; Ni, L.; Sun, J.; Liu, B.; Rao, P.; Lv, X. Monascus yellow, red and orange pigments from red yeast rice ameliorate lipid metabolic disorders and gut microbiota dysbiosis in Wistar rats fed on a high-fat diet. Food Funct. 2019, 10, 1073–1084. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lee, C.L.; Wen, J.Y.; Hsu, Y.W.; Pan, T.M. The blood lipid regulation of Monascus-produced monascin and ankaflavin via the suppression of low-density lipoprotein cholesterol assembly and stimulation of apolipoprotein A1 expression in liver. J. Microbiol. Immunol. Infect. 2018, 51, 27–37. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wu, L.; Zhou, K.; Chen, F.; Chen, G.; Yu, Y.; Lv, X.; Zhang, W.; Rao, P.; Ni, L. Comparative Study on the Antioxidant Activity of Monascus Yellow Pigments From Two Different Types of Hongqu-Functional Qu and Coloring Qu. Front. Microbiol. 2021, 12, 715295. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wu, S.; Sun, Y.; Chen, D.; Liu, H.; Li, Z.; Chen, M.; Wang, C.; Cheng, L.; Guo, Q.; Peng, X. The noncovalent conjugations of human serum albumin (HSA) with MS/AK and the effect on anti-oxidant capacity as well as anti-glycation activity of Monascus yellow pigments. Food Funct. 2021, 12, 3692–3704. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wu, S.; Wang, W.; Lu, J.; Deng, W.; Zhao, N.; Sun, Y.; Liu, H.; Li, Z.; Chen, M.; Cheng, L.; et al. Binding of ankaflavin with bovine serum albumin (BSA) in the presence of carrageenan and protective effects of Monascus yellow pigments against oxidative damage to BSA after forming a complex with carrageenan. Food Funct. 2023, 14, 2459–2471. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- El-Far, S.W.; Helmy, M.W.; Khattab, S.N.; Bekhit, A.A.; Hussein, A.A.; Elzoghby, A.O. Phytosomal bilayer-enveloped casein micelles for codelivery of monascus yellow pigments and resveratrol to breast cancer. Nanomedicine 2018, 13, 481–499. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lu, J.; Dong, C.; Cheng, Y.; Zhang, M.; Pang, Q.; Zhou, S.; Yang, B.; Peng, X.; Wang, C.; Wu, S. Ankaflavin and Monascin Prevent Fibrillogenesis of Hen Egg White Lysozyme: Focus on Noncovalent and Covalent Interactions. J. Phys. Chem. B 2024, 128, 10051–10062. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wu, S.; Dong, C.; Zhang, M.; Cheng, Y.; Cao, X.; Yang, B.; Li, C.; Peng, X. Revealing the hypoglycemic effect of red yeast rice: Perspectives from the inhibition of α-glucosidase and the anti-glycation capability by ankaflavin and monascin. Foods 2024, 13, 1573. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hsu, W.H.; Lee, B.H.; Lu, I.J.; Pan, T.M. Ankaflavin and monascin regulate endothelial adhesion molecules and endothelial NO synthase (eNOS) expression induced by tumor necrosis factor-α (TNF-α) in human umbilical vein endothelial cells (HUVECs). J. Agric. Food Chem. 2012, 60, 1666–1672. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gordon, R.Y.; Cooperman, T. Marked variability of monacolin levels in commercial red yeast rice products. JAMA Intern. Med. 2010, 170, 1722–1723. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Banach, M.; Norata, G.D. Rhabdomyolysis or severe acute hepatitis associated with the use of red yeast rice extracts: An update from the adverse event reporting systems. Curr. Atheroscler. Rep. 2023, 25, 859–869. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kurnik, M.; Markelj, T.Ž.B.; Hudournik, B.M.M.; Podbregar, M. Fulminant red yeast rice-associated rhabdomyolysis with acute liver injury and hyperkalemia treated with extracorporeal blood purification. Drug Healthc. Patient Saf. 2025, 17, 109–120. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Norata, G.D.; Banach, M. The impact of red yeast rice extract use on the occurrence of muscle symptoms and liver dysfunction: An update from the adverse event reporting systems and available meta-analyses. Nutrients 2024, 16, 444. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yang, H.T.; Lin, S.H.; Huang, S.Y.; Chou, H. Acute administration of red yeast rice (Monascus purpureus) depletes tissue coenzyme Q10 levels in ICR mice. Br. J. Nutr. 2005, 93, 131–135. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Rigillo, G.; Baini, G.; Bruni, R.; Puja, G.; Miraldi, E.; Pani, L.; Tascedda, F.; Biagi, M. Red yeast rice or lovastatin? A comparative evaluation of safety and efficacy through a multifaceted approach. Phytother. Res. 2025, 39, 264–281. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fogacci, F.; Banach, M.; Mikhailidis, D.P.; Bruckert, E.; Toth, P.P.; Watts, G.F.; Reiner, Ž.; Mancini, J.; Rizzo, M.; Mitchenko, O.; et al. Safety of red yeast rice supplementation: A systematic review and meta-analysis of randomized controlled trials. Pharmacol. Res. 2019, 143, 1–16. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhu, B.; Qi, F.; Wu, J.; Yin, G.; Hua, J.; Zhang, Q.; Qin, L. Red Yeast Rice: A Systematic Review of the Traditional Uses, Chemistry, Pharmacology, and Quality Control of an Important Chinese Folk Medicine. Front. Pharmacol. 2019, 10, 1449. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nguyen, T.; Karl, M.; Santini, A. Red yeast rice. Foods 2017, 6, 19. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Minamizuka, T.; Koshizaka, M.; Shoji, M.; Yamaga, M.; Hayashi, A.; Ide, K.; Ide, S.; Kitamoto, T.; Sakamoto, K.; Hattori, A.; et al. Low dose red yeast rice with monacolin K lowers LDL cholesterol and blood pressure in Japanese with mild dyslipidemia: A multicenter, randomized trial. Asia Pac. J. Clin. Nutr. 2021, 30, 424–435. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cicero, A.F.G.; Fogacci, F.; Zambon, A. Red Yeast Rice for Hypercholesterolemia: JACC Focus Seminar. J. Am. Coll. Cardiol. 2021, 77, 620–628. [Google Scholar] [PubMed]
- Lin, T.S.; Chiu, S.H.; Chen, C.C.; Lin, C.H. Investigation of monacolin K, yellow pigments, and citrinin production capabilities of Monascus purpureus and Monascus ruber (Monascus pilosus). J. Food Drug Anal. 2023, 31, 85–94. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lee, H.; Do, B.; Kwon, H. Effect of red yeast rice on the growth of male SD rats: A 90-day feeding study. Toxicol. Res. 2025, 41, 503–513. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yang, P.X.; You, C.R.; Lin, Y.H.; Wang, C.S.; Hsu, Y.W.; Pan, T.M.; Lee, C.L. Effects of Monascus pilosus SWM 008-fermented red mold rice and its functional components on gut microbiota and metabolic health in rats. Foods 2025, 14, 651. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gao, F.; Cheng, C.; Li, R.; Chen, Z.; Tang, K.; Du, G. The role of Akkermansia muciniphila in maintaining health: A bibliometric study. Front. Med. 2025, 12, 1484656. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gao, W.; Chen, X.; Wu, S.; Jin, L.; Chen, X.; Mao, G.; Wan, X.; Xing, W. Monascus red pigments alleviate high-fat and high-sugar diet-induced NAFLD in mice by modulating the gut microbiota and metabolites. Food Sci. Nutr. 2024, 12, 5762–5775. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Huang, Y.P.; Li, P.; Du, T.; Du, X.J.; Wang, S. Protective effect and mechanism of Monascus-fermented red yeast rice against colitis caused by Salmonella enterica serotype Typhimurium ATCC 14028. Food Funct. 2020, 11, 6363–6375. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xue, F.; Zhu, R.; Li, J.; Liu, Z.; Niu, L.; Chen, W.; Wang, C.; Zheng, J. Monascus yellow pigments ameliorate hyperuricemia via dual mechanisms: Xanthine oxidase inhibition and uric acid transporter modulation. Foods 2025, 14, 2765. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Shaleha, R.; Yuliana, A.; Amin, S.; Levita, J.; Sumiwi, S. Monascus purpureus red yeast rice: A review of the in vitro and in vivo pharmacological activities, studies in humans, and case reports. Clin. Pharmacol. Adv. Appl. 2025, 17, 269–289. [Google Scholar] [CrossRef] [Scilit] [PubMed]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.