


Simple Summary
Gyrfalcons (Falco rusticolus) begin breeding exceptionally early in the Arctic, often while nesting sites remain surrounded or covered by snow. We compared breeding performance on the Yamal Peninsula, Russia, during a late, cold spring in 2024 and an earlier, warmer spring in 2025. The study covered natural tree nests, artificial nests mounted in trees, rock nests, and raven-built bridge nests. The proportion of monitored territories occupied by Gyrfalcons was similar between years, but more occupied territories progressed to egg laying in 2025, and hatching and later nesting success were much higher. Minimum confirmed productivity was also higher in 2025, although several late 2024 broods could not be followed until young reached the 36-day age used to confirm success. Permanent-quadrat surveys showed no interannual difference in ptarmigan pellet occurrence, an indirect index of relative winter–spring prey occurrence. Direct observations of eggs laid in snow or ice accumulated within raven-built bridge nests showed how persistent snow can make an existing nest temporarily unsuitable. The results show that prey, spring conditions, and nest-site condition should be monitored together, but with only two years of data, we cannot establish that spring weather caused the difference in breeding performance.
Abstract
Spring conditions may influence reproduction in the Gyrfalcon, Falco rusticolus, but their effects are difficult to separate from prey variation. We compared 66 nesting territories in 2024 and 69 in 2025 across natural tree nests, artificial nests mounted in trees, rock nests, and raven-built bridge nests on the Yamal Peninsula, Russia. Occupancy did not differ between years (35/66 vs. 40/69; Fisher’s exact test, p = 0.606). The proportion of occupied territories with a confirmed nesting attempt was higher in 2025 but not statistically significant (18/35 vs. 30/40; p = 0.053). Hatching success was higher in 2025 (7/15 vs. 26/29; p = 0.003), as was apparent nesting success among attempts with known outcomes (3/11 vs. 19/24; p = 0.007). Exact paired comparisons of permanent quadrats detected no interannual difference in ptarmigan pellet occurrence. The reproductive contrast coincided with earlier warming and snowmelt in 2025. Direct observations of eggs laid in snow or ice accumulated within raven-built bridge nests illustrated a nest-scale pathway to early failure. Although this two-year comparison documents an association between spring conditions and breeding performance rather than demonstrating causality, the results show why spring conditions, prey, and functional nest-site availability should be evaluated together in Gyrfalcon monitoring and conservation.
1. Introduction
Few Arctic birds begin reproduction as early as Gyrfalcons. Egg laying and incubation can overlap deep snow, recurrent freezing, and spring snowstorms, creating a narrow period in which nest condition, food supply, and parental performance must align. More broadly, climate warming is altering Arctic snow regimes, seasonal timing, species distributions, and trophic interactions, but biological responses are stage-specific and cannot be inferred from mean annual temperature alone [1,2,3]. Weather can affect raptors directly through exposure of eggs and young and indirectly through adult foraging efficiency, prey accessibility, and food delivery [4,5,6]. Accordingly, occupancy, nesting attempts, hatching success, nesting success, and productivity should be treated as distinct components of breeding performance [7,8,9].
The Gyrfalcon, Falco rusticolus, is a circumpolar, cold-adapted raptor whose early breeding ecology is closely linked to ptarmigan, Lagopus spp. Ptarmigan dominate the diet in most studied populations and are especially important from courtship through hatching, before many alternative prey become abundant or accessible [10,11,12]. Variation in ptarmigan abundance can therefore influence territory occupancy, egg laying, timing, and reproductive output [12,13]. Alternative prey, habitat context, and local environmental conditions can modify this relationship [13,14,15], so food supply should be evaluated together with weather and snow conditions.
Gyrfalcon laying and incubation may begin while temperatures remain below freezing and nest substrates are still snow-covered [6,16,17]. Severe weather has been associated with early nestling mortality [17] and affects reproduction in other Arctic raptors [5,18]. Weather may act through several pathways, including adult condition and prey accessibility, but for an early-breeding falcon it may also determine whether an existing nest structure provides a dry, usable incubation site. Franke [6] therefore argued that Gyrfalcon studies under climate change should assess weather and food supply simultaneously.
Nest-site availability adds another constraint. Like other falcons, Gyrfalcons do not build their own nests and depend on cliff ledges, tree nests, artificial platforms, or stick nests built by other birds, especially the Common Raven (Corvus corax) [11,16,17]. A nesting territory may therefore be occupied even when no functional nest site is available. In snow-rich springs, a nest cup covered by snow or ice may remain unsuitable during laying and incubation despite the presence of an otherwise intact nest structure.
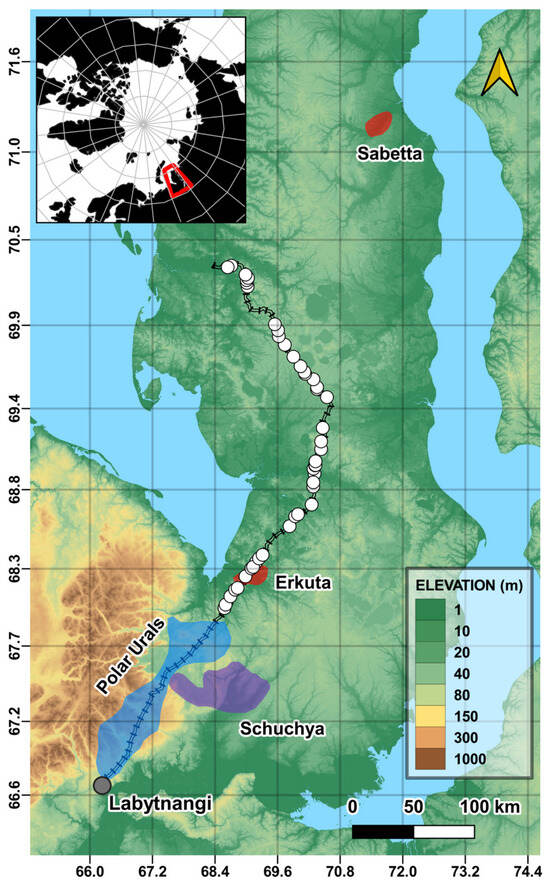
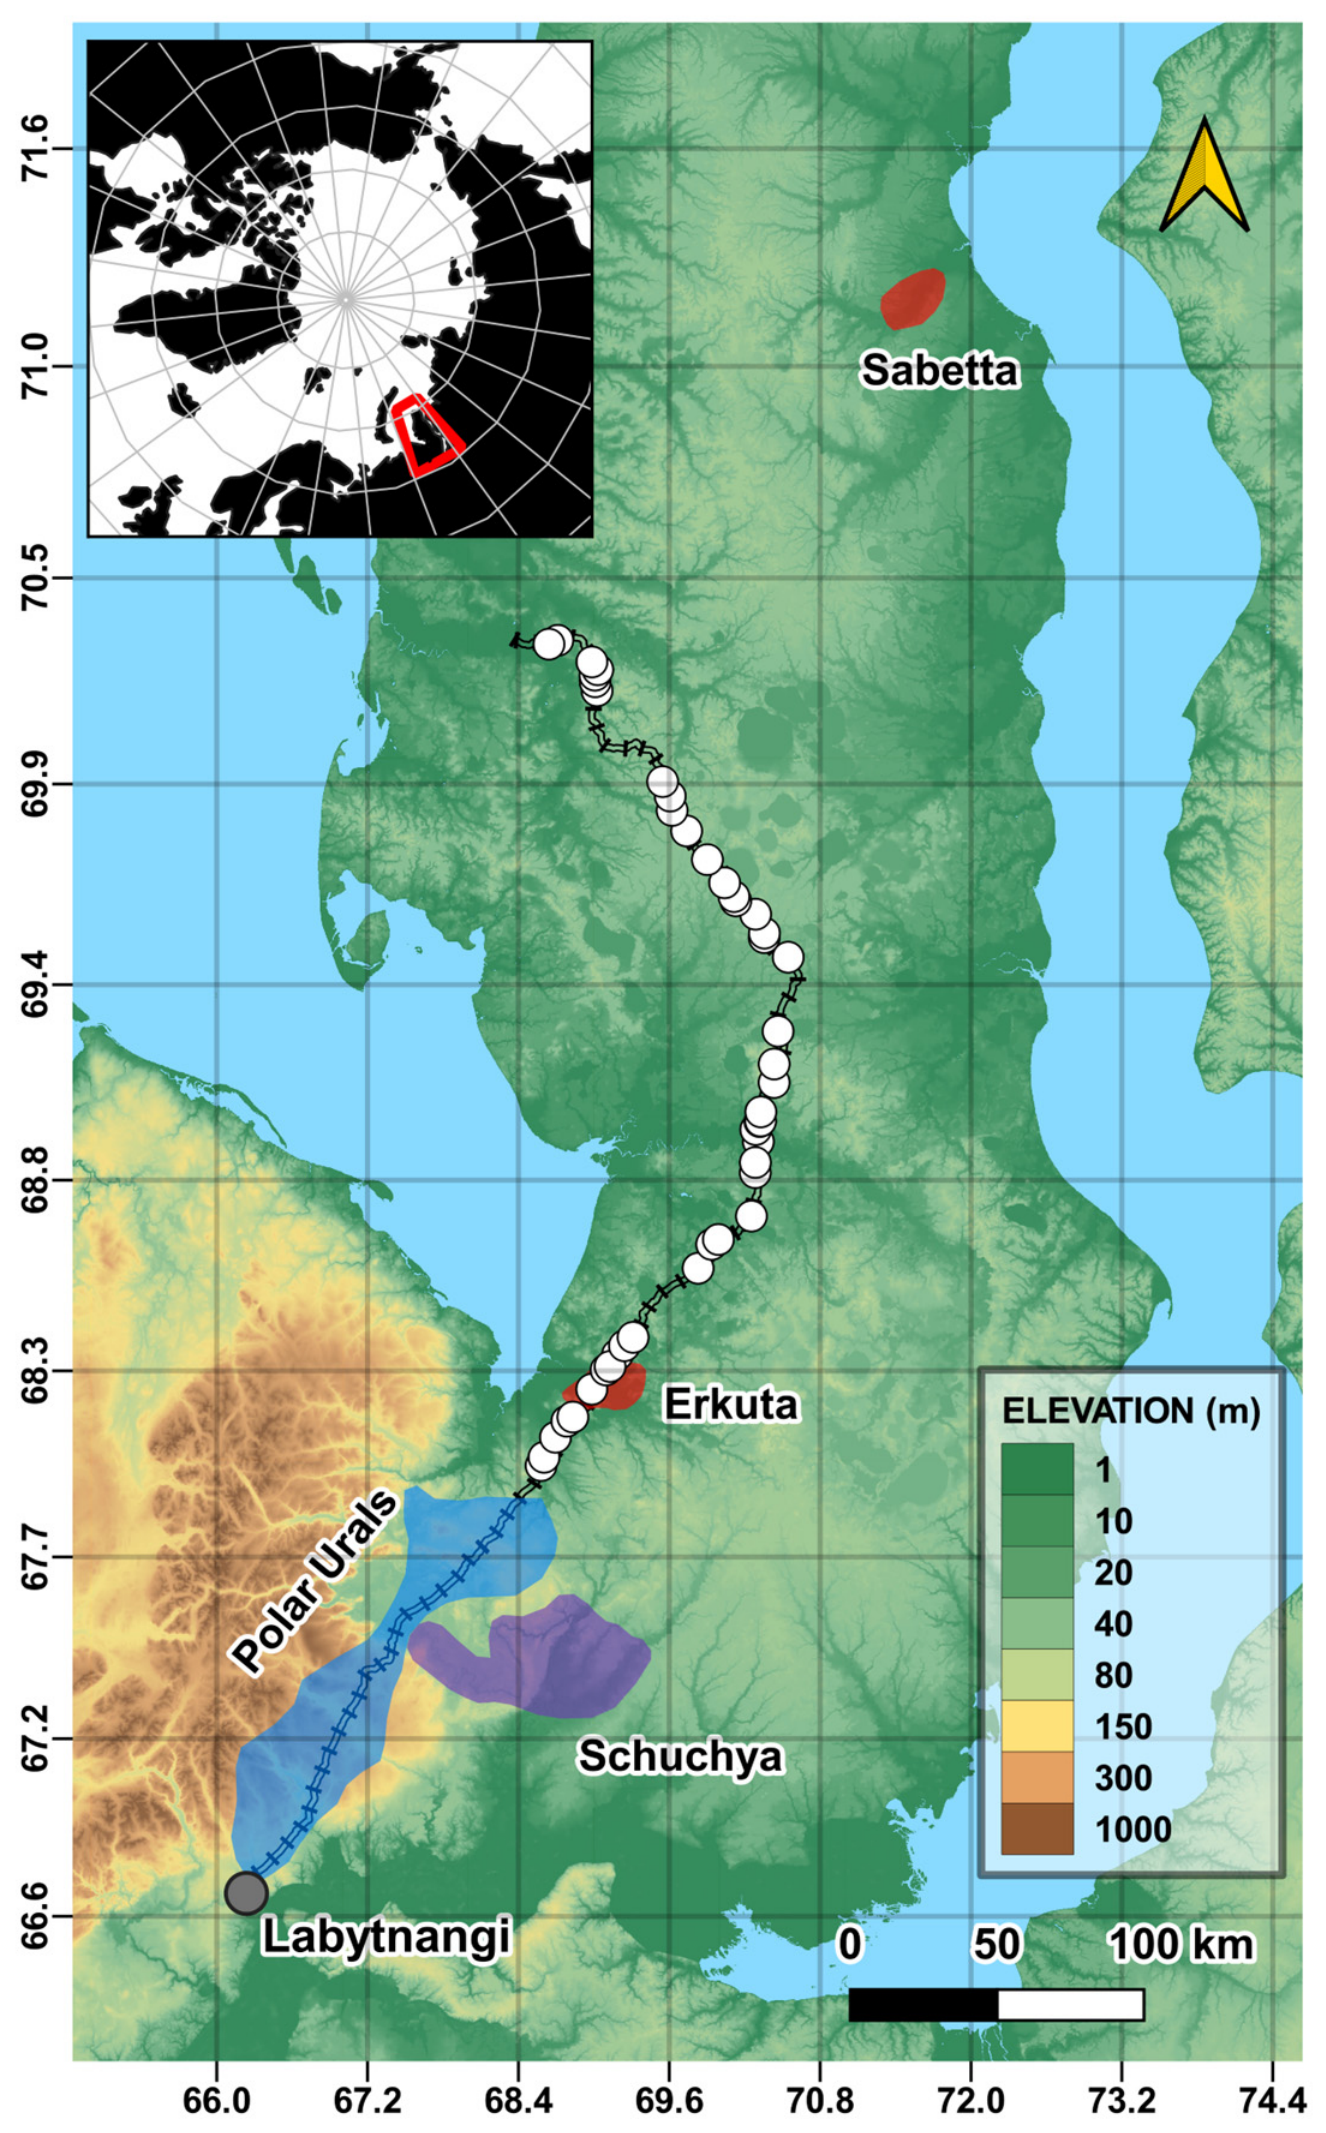
The Yamal Peninsula in north-western Siberia provides a suitable setting for examining these relationships because it spans forest-tundra, shrub tundra, typical tundra, and arctic tundra [19,20]. In the southern and south-western part of the Gyrfalcon breeding range on Yamal, Gyrfalcons use natural tree nests, artificial nests mounted in trees, and rock nests, including in the Schuchya River basin and the eastern foothills of the Polar Urals [21]. Farther north, where natural elevated nesting substrates become scarce, railway bridges along the Obskaya–Karskaya railway support raven-built stick nests used by Gyrfalcons [22]. The location of the three monitored breeding areas is shown in Figure 1.
Figure 1.
Location of the three Gyrfalcon breeding areas monitored on the Yamal Peninsula, Russia, in 2024–2025: the Schuchya River basin (violet), the eastern foothills of the Polar Urals (blue), and railway bridges along the Obskaya–Karskaya railway. White circles indicate checked railway bridges. The red outline in the inset indicates the location of the Yamal Peninsula within the Arctic. Red polygons indicate the Erkuta and Sabetta field sites, where permanent ptarmigan pellet-monitoring plots provided indices of relative prey occurrence.
We compared Gyrfalcon breeding performance during two adjacent breeding seasons, 2024 and 2025, across three Yamal breeding areas encompassing natural tree nests, artificial nests mounted in trees, rock nests, and raven-built bridge nests. The seasons differed markedly in spring snow and temperature conditions during laying, incubation, and early hatching. We used this contrast to evaluate how interannual differences in reproduction aligned with spring conditions and with the relative occurrence of ptarmigan, the principal prey.
Specifically, we compared nesting-territory occupancy, confirmed nesting attempts, hatching success, apparent nesting success, minimum productivity, brood size at success, and hatching phenology. We also compared ptarmigan pellet occurrence in permanent quadrats at Erkuta in south-western Yamal and Sabetta in north-eastern Yamal. Finally, we examined snow- and ice-associated egg laying at bridge nests as a possible nest-scale mechanism linking persistent spring snow to early breeding failure.
By combining monitoring of natural and infrastructure-associated nesting sites with regional spring-weather data, hatching phenology, and standardized ptarmigan indices, this study asks where in the reproductive cycle the two years differed and which mechanisms are directly supported by the observations. This question is directly relevant to avian conservation in the Anthropocene, where climate change, infrastructure development, and evidence-based management increasingly need to be considered together rather than as separate conservation issues.
2. Materials and Methods
2.1. Study Area
The study was conducted on the Yamal Peninsula, north-western Siberia, Russia. Yamal is a low-relief Arctic peninsula underlain by continuous permafrost. It extends from forest-tundra and shrub tundra in the south to typical and arctic tundra farther north. The landscape is dissected by broad river valleys, lakes, and wetlands. Vegetation changes northward from low-shrub tundra to sedge-, dwarf-shrub-, and moss-dominated tundra [19,20]. The regional climate is characterized by long severe winters and short cool summers [23,24].
We monitored Gyrfalcon nesting territories in three breeding areas on Yamal: the Schuchya River basin, the eastern foothills of the Polar Urals, and railway bridges along the Obskaya–Karskaya railway (Figure 1). These areas differed in nesting substrate. In the Polar Urals, all monitored nests were on rocks. In the Schuchya River basin, all monitored nests except one were in trees, and the area included a long-term network of tree-mounted artificial nests installed before the present study [21]. Along the railway, monitored nests were stick nests built by Common Ravens (Corvus corax) on bridge structures [22]. The Obskaya–Karskaya railway is a single-track industrial railway crossing the Yamal Peninsula from south to north. For the 2024–2025 comparison, a bridge was treated as a potential Gyrfalcon nesting territory and included among checked territories when at least one raven-built stick nest was present in that year.
2.2. Nest Monitoring
We compared two breeding seasons, 2024 and 2025. In total, 66 Gyrfalcon nesting territories were checked in 2024 and 69 in 2025. These included 27 territories in the Schuchya River basin in both years, 8 and 10 territories in the Polar Urals, and 31 and 32 bridge nesting territories in 2024 and 2025, respectively.
In all three breeding areas, nesting territories were checked by direct inspection, ground-based observations, photographs, and unmanned aerial vehicles (UAVs, DJI Mavic 3 Pro quadcopter, SZ DJI Technology Co., Ltd., Shenzhen, China), when needed. We checked nests built by other bird species that were suitable for Gyrfalcon nesting and recorded adult Gyrfalcons, territorial behavior, incubating birds, eggs, young, fledglings, failed eggs, and dead young. Photographs and UAVs were used when nest contents could not be assessed reliably from the ground. Camera traps (SEELOCK S308W; Shenzhen Chaonuo Technology Co., Ltd., Shenzhen, China) were used on railway bridges where they could be safely attached to the bridge structure.
Railway bridges were checked on 6–8 May and 1–2 July 2024, and on 17–19 May and 1–2 July 2025. Surveys followed the long-term bridge-monitoring protocol for the Obskaya–Karskaya railway [22]. Bridges were accessed using a self-propelled railway vehicle (the ASE-1 service rail car, Kalugaputmash, Kaluga, Russia), designed for the rapid deployment of railway maintenance personnel. At each bridge, at least two observers inspected the bridge structure from the ground.
Known rock nests in the Polar Urals were checked twice in both years. The first checks were conducted in May and the second checks in the second half of June. Spring surveys were conducted using a Trecol-Khaski (6×6 low-pressure tire all-terrain vehicle, LLC STC TRECOL, Lyubertsy, Russia) and snowmobiles (Ski-Doo 900 ACE by BRP, Valcourt, QC, Canada; and Yamaha Venture Multi Purpose by Yamaha Motor Company, Iwata, Japan). June surveys were conducted using a Trecol-Khaski.
Known nesting territories in the Schuchya River basin were checked from 15 June to 3 August in both years. Surveys were conducted along the Schuchya River and its tributaries by kayak and on foot.
These schedules meant that bridge and Polar Ural surveys covered laying or incubation as well as later nest stages. In Schuchya, first checks were mostly conducted after hatching had begun, so early failed nesting attempts were less likely to be detected. Survey timing within Schuchya was nevertheless comparable between years.
2.3. Breeding Definitions
We followed standard raptor terminology as closely as possible [7,8,9]. A territory was considered occupied when one or more Gyrfalcons were recorded at or near the known nesting site, or when fresh evidence of current-year Gyrfalcon use was present there. A nesting attempt was defined by evidence that egg laying had occurred, including eggs, an adult in incubation posture associated with a nest, or young recorded later in the same season at the same territory.
Clutch size was summarized only when eggs were directly visible and countable. Cases in which eggs were laid on thick snow or ice covering raven-built nests on bridges were retained as nesting attempts and, when outcome was known, as failed hatching outcomes. These cases were excluded from clutch-size summaries because they likely represented interrupted or rapidly failed laying attempts rather than completed clutches.
Hatching success was defined as hatching of at least one young and was calculated only for attempts with known hatching outcome. Apparent nesting success was defined as the proportion of attempts with known outcome in which at least one young reached the minimum acceptable age for assessing success; for Gyrfalcons, this threshold is 36 days [8]. Attempts last observed before young reached 36 days, and for which failure was not subsequently confirmed, were classified as having unknown outcome and excluded from apparent nesting-success calculations. The number of young reaching at least 36 days was treated as minimum confirmed productivity, and brood size at success was calculated per successful nest.
2.4. Hatching Dates
First-hatching dates were estimated for broods in which nestling age could be assessed from field observations, photographs, UAV images, or repeated visits. For each brood, the first-hatching date was calculated as the observation date minus the estimated age of the oldest young. Nestling age was estimated from body size and plumage development following Anderson et al. [25]. Broods with insufficient information for age estimation were excluded from hatching-date summaries.
2.5. Weather Data
Spring weather was characterized using the Erkuta field station in south-western Yamal, the nearest continuous high-resolution record available for the monitored breeding areas. Erkuta lies within the southern railway study area, close to several monitored bridges and approximately 100 km from the Schuchya breeding area. Air temperature was recorded with a HOBO U30 USB weather station (Onset Computer Corporation, Bourne, MA, USA), and snow depth with a custom weather station built around a Campbell Scientific CR1000 data logger (Campbell Scientific, Logan, UT, USA). We used daily air-temperature and snow-depth data for April–June. Daily mean and minimum air temperatures were calculated, and positive degree-days were summed from daily mean temperatures above 0 °C. Conditions were summarized by half-month periods and for 15 May–15 June, which overlapped incubation and early hatching at many nests. These data were treated as a regional environmental reference rather than as measurements at individual nests.
Snow depth was summarized as daily median depth after correction of the snow-sensor offset (20 cm). The timing of the main snowmelt transition was identified from the corrected daily snow-depth series.
2.6. Ptarmigan Pellet Index
We used ptarmigan (Lagopus spp.) pellet occurrence in permanent quadrats as an index of relative winter–spring ptarmigan occurrence. Pellets were counted post-snowmelt and removed after counting [26].
Pellet surveys were conducted at the long-term field sites Erkuta (68.2° N, 69.1° E), south-western Yamal, and Sabetta (71.2° N, 71.5° E), north-eastern Yamal (Figure 1). Erkuta was the principal regional prey index because it was closest to the Gyrfalcon breeding areas; Sabetta provided an additional northern index. The permanent monitoring networks comprised 576 quadrats at Erkuta and 288 at Sabetta. Permanent 50 × 50 cm quadrats were distributed across approximately 38 km2 at Erkuta and 18 km2 at Sabetta and spanned the main local habitat types. Each quadrat was scored as 1 when at least one ptarmigan pellet was present and 0 otherwise. Formal interannual comparisons used only permanent quadrats with valid post-snowmelt observations in both years.
2.7. Statistical Analysis
For Gyrfalcons, we summarized occupancy, nesting attempts, hatching success, apparent nesting success, clutch size, hatching phenology, and minimum confirmed productivity by breeding area and year. Occupancy was calculated as occupied territories divided by checked territories. Clutch size and brood size at success were reported as mean ± SE when n > 1 and as individual values when n = 1.
Annual differences in occupancy, nesting-attempt rate, hatching success, and apparent nesting success were evaluated using two-sided Fisher’s exact tests [27]. Nesting-attempt rate was calculated among occupied territories, whereas hatching and apparent nesting success were calculated only among attempts with known respective outcomes. Because early failed attempts were less detectable in Schuchya, the hatching- and apparent nesting-success analyses were repeated after restricting the dataset to railway bridges and the Polar Urals. For ptarmigan pellet occurrence, we calculated annual proportions and exact 95% Clopper–Pearson confidence intervals; interannual comparisons at each site used exact McNemar tests restricted to permanent quadrats with valid observations in both years [27]. Weather variables were summarized descriptively because only two breeding seasons were compared. All statistical analyses were performed in R version 4.6.0 (R Core Team, R Foundation for Statistical Computing, Vienna, Austria).
3. Results
3.1. Gyrfalcon Nesting Territory Occupancy and Nesting Attempts
The comparison included 66 checked Gyrfalcon nesting territories in 2024 and 69 in 2025: 27 territories in the Schuchya River basin in both years, 8 and 10 in the Polar Urals, and 31 and 32 bridge nesting territories, respectively.
Occupancy was 35/66 (53.0%) in 2024 and 40/69 (58.0%) in 2025 and did not differ significantly between years (two-sided Fisher’s exact test, p = 0.606; Table 1). Area-specific occupancy values are shown in Table 1.
Table 1.
Nesting-territory occupancy, nesting attempts, hatching success, and apparent nesting success of Gyrfalcons in the three breeding areas distinguished on Yamal, 2024–2025.
The proportion of occupied territories with a confirmed nesting attempt increased from 18/35 in 2024 to 30/40 in 2025, but the comparison was not statistically significant at the 0.05 level (two-sided Fisher’s exact test, p = 0.053). The numerical increase occurred in all three breeding areas (Table 1).
3.2. Hatching Success
Hatching success was significantly higher in 2025 than in 2024: at least one young hatched in 7/15 attempts with known hatching outcome in 2024 and 26/29 in 2025 (two-sided Fisher’s exact test, p = 0.003).
The contrast remained significant when the analysis was restricted to railway bridges and the Polar Urals, where surveys covered laying or incubation: hatching success increased from 2/10 in 2024 to 14/17 in 2025 (p = 0.003). Schuchya values were 5/5 and 12/12, but early failed attempts were less detectable there because field checks started later.
3.3. Apparent Nesting Success and Productivity
Apparent nesting success among attempts with known outcome was also significantly higher in 2025: 3/11 attempts were successful in 2024 and 19/24 in 2025 (two-sided Fisher’s exact test, p = 0.007). When Schuchya was excluded, the contrast was stronger, increasing from 0/8 on bridges and in the Polar Urals in 2024 to 13/17 in 2025 (p < 0.001).
Minimum confirmed productivity increased from 4 young reaching at least 36 days in 2024 to 50 in 2025 (Table 2). In 2024, two bridge broods had hatched but were only 28 and 29 days old at the final standardized July visit and therefore had not yet reached the 36-day threshold; their later outcomes remained unknown. All four confirmed young in 2024 were recorded in Schuchya; in 2025, 12 were recorded in Schuchya, 13 in the Polar Urals, and 25 on railway bridges.
Table 2.
Clutch size and productivity of Gyrfalcons in the three breeding areas distinguished on Yamal, 2024–2025.
Clutch size was available only for directly counted clutches and was unevenly represented among breeding areas. On railway bridges, where spring checks were most consistent, mean countable clutch size was 3.25 ± 0.48 eggs in 2024 and 3.83 ± 0.17 eggs in 2025.
3.4. Hatching Phenology
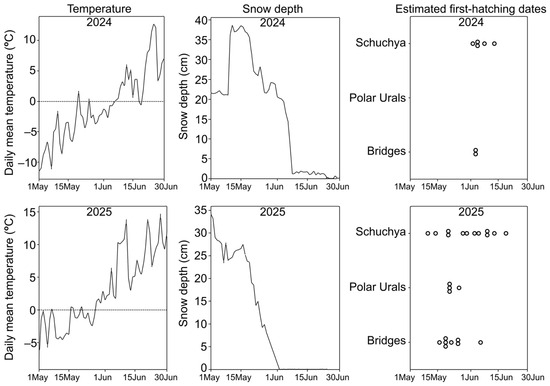
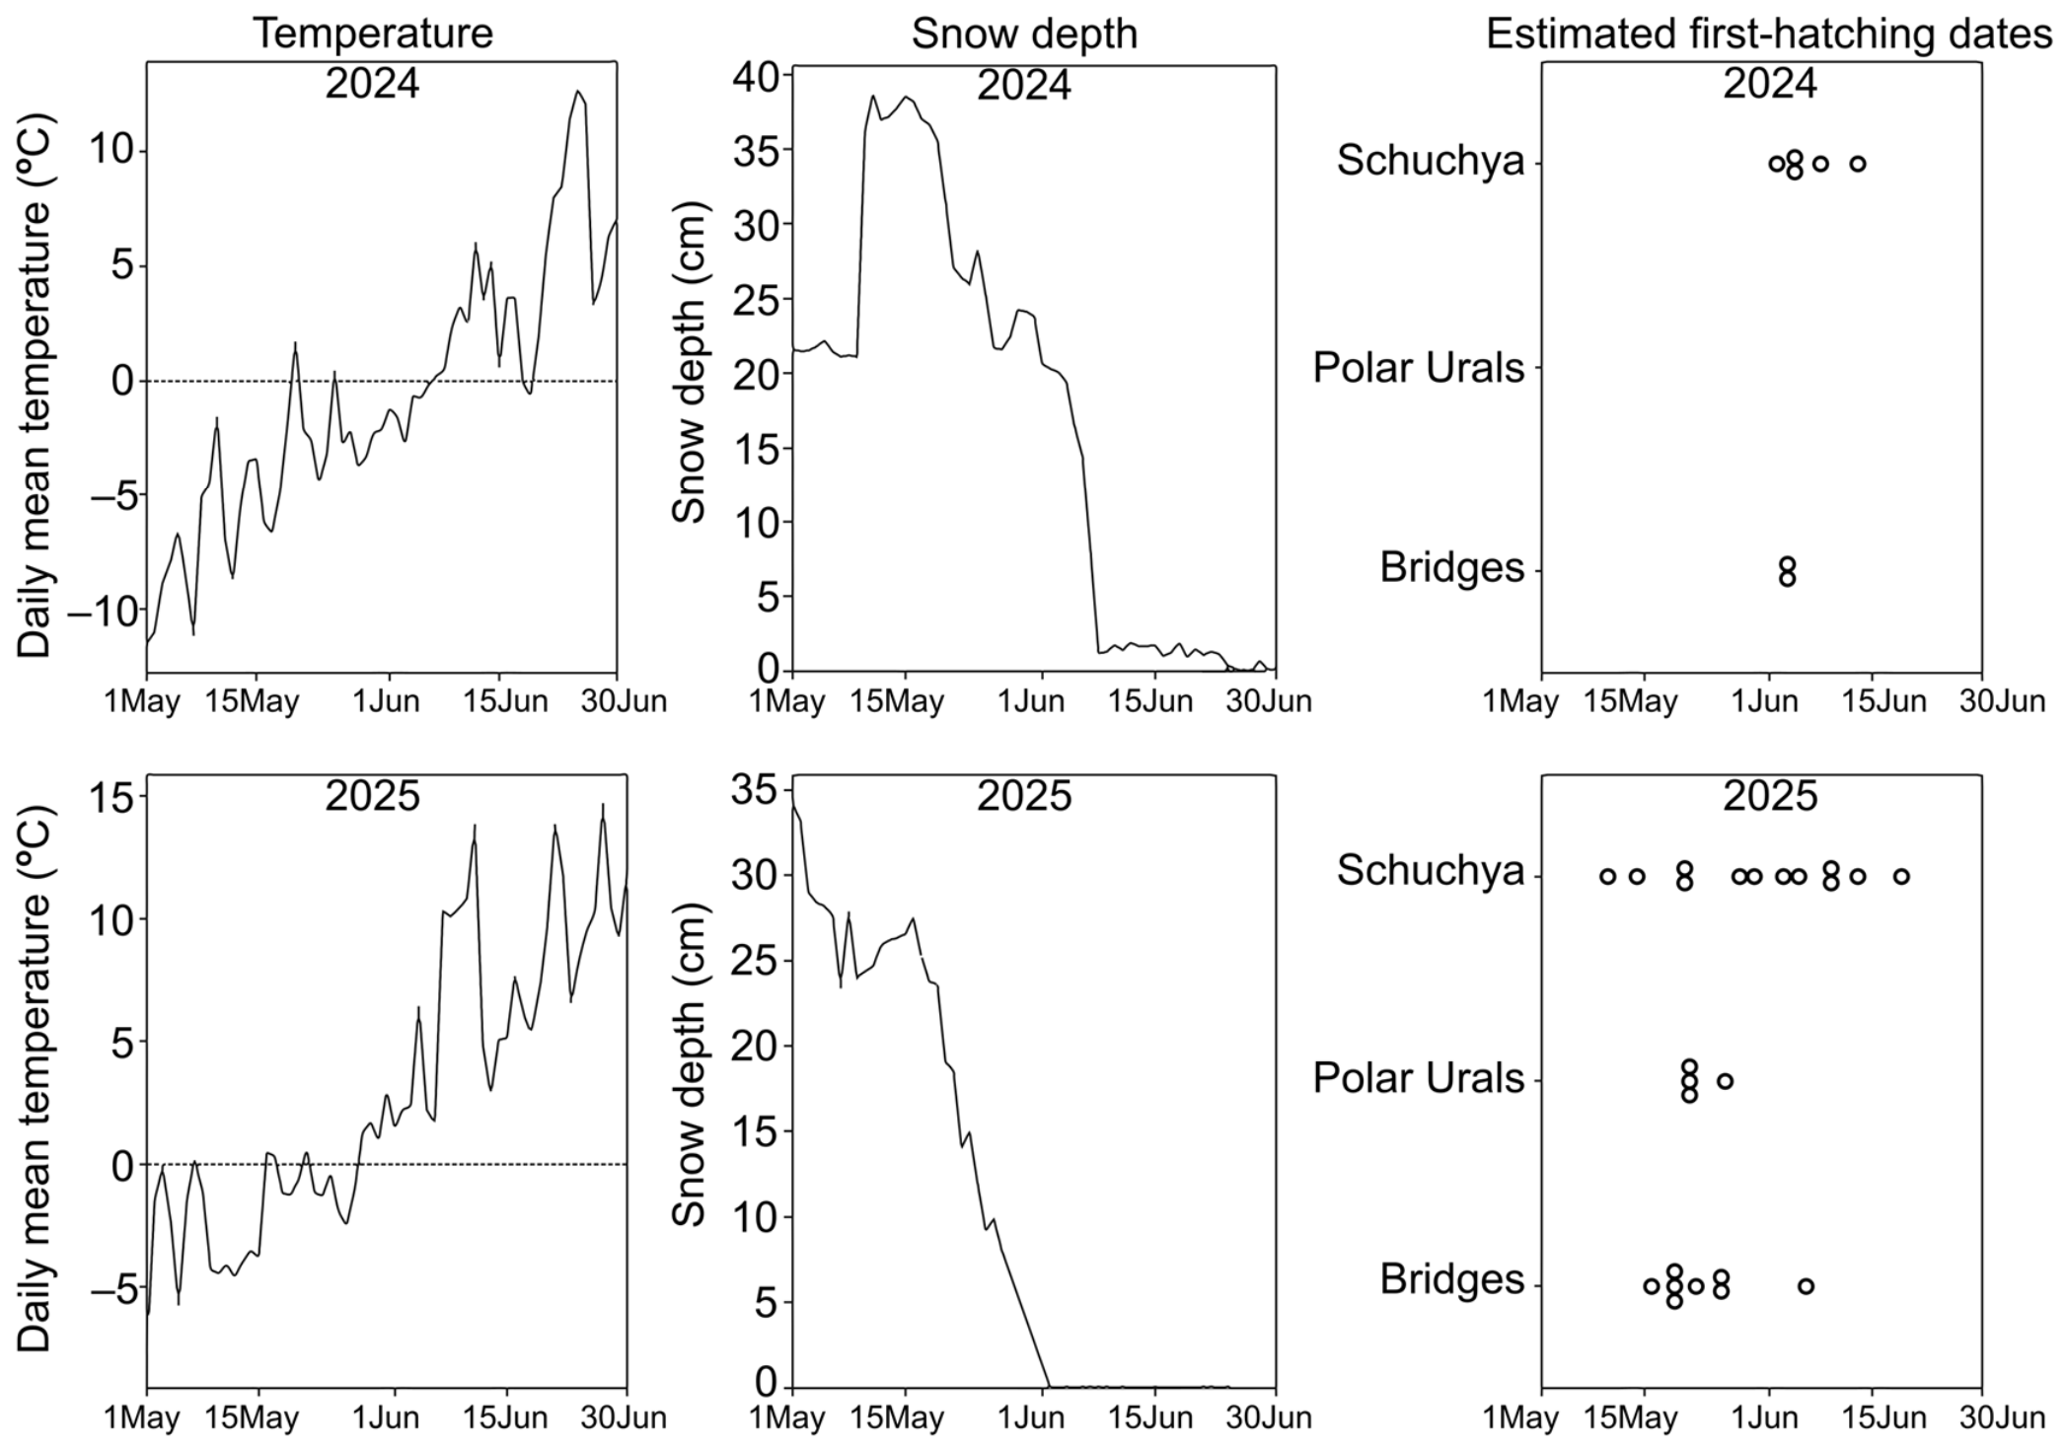
Estimated first-hatching dates were later in 2024 than in 2025 (Figure 2). Dates ranged from 2 to 13 June in 2024, with a median of 4 June, and from 10 May to 19 June in 2025, with a median of 22 May.
Figure 2.
Spring temperature, snow depth, and estimated first-hatching dates of Gyrfalcons on Yamal in 2024 and 2025. Rows show years; columns show daily mean air temperature, daily median snow depth at the Erkuta field site, and estimated first-hatching dates. The dashed horizontal line in the temperature panels marks 0 °C. Open circles indicate estimated first-hatching dates for individual broods in the three Gyrfalcon breeding areas distinguished in this study: Schuchya River basin, eastern foothills of the Polar Urals, and railway bridges along the Obskaya–Karskaya railway.
On railway bridges, first hatching was estimated only for two broods in 2024, on 3 and 4 June. In 2025, first hatching was estimated for nine bridge broods. Dates ranged from 16 May to 6 June, with a median of 20 May. In the Polar Urals, no brood hatched in the monitored 2024 attempts, whereas the five estimated first-hatching dates in 2025 ranged from 20 to 26 May, with a median of 22 May. In Schuchya, first hatching was estimated for five broods in 2024 and 12 broods in 2025. Dates ranged from 2 to 13 June in 2024, with a median of 5 June, and from 10 May to 19 June in 2025, with a median of 1 June.
3.5. Ptarmigan Pellet Indices
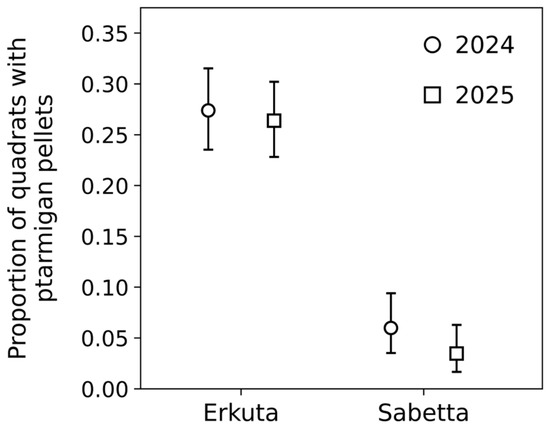
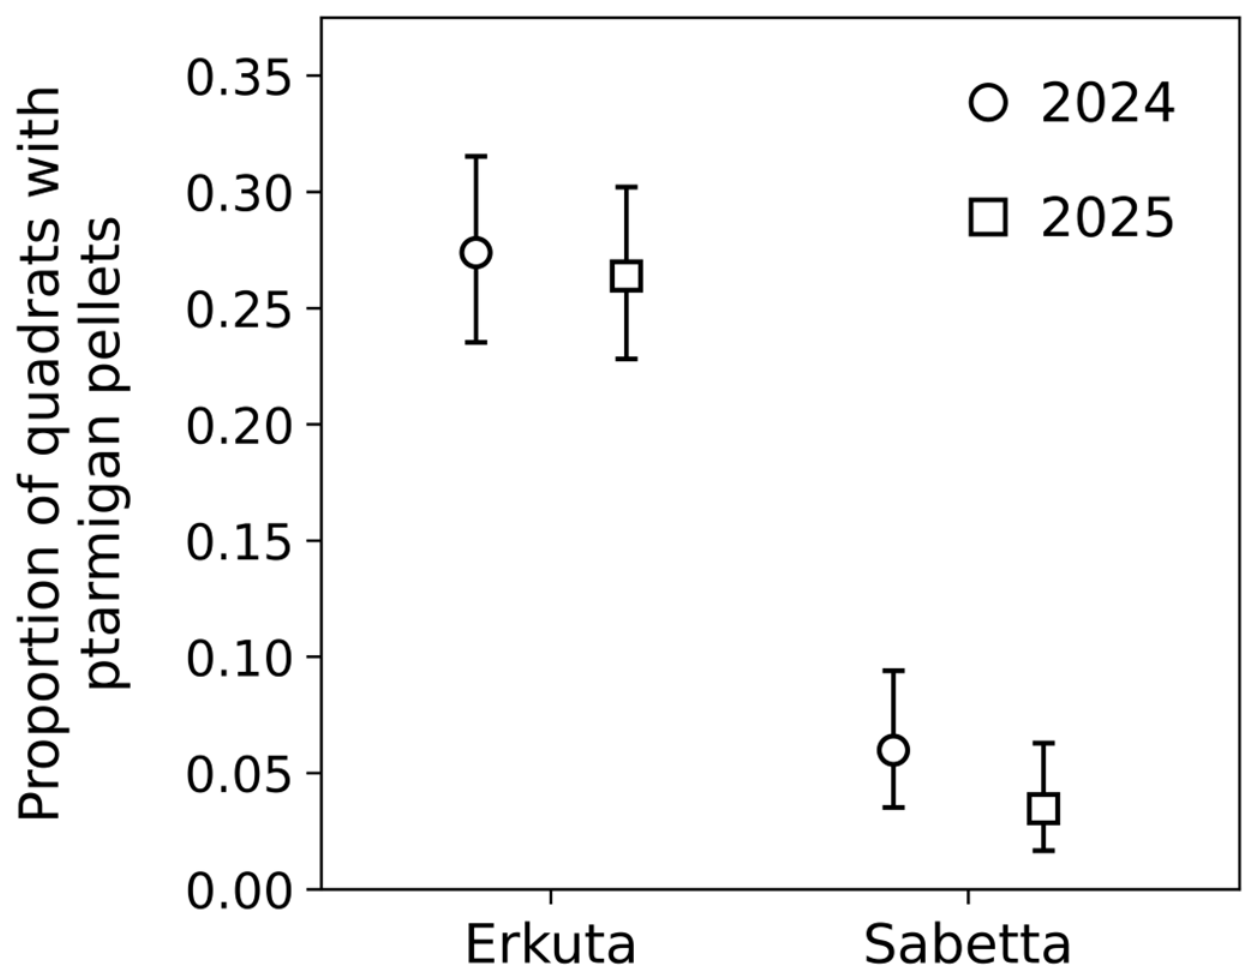
Ptarmigan pellet occurrence in permanent quadrats was comparable between years (Figure 3). At Erkuta, pellets were recorded in 137/500 assessable quadrats in 2024 and 151/572 in 2025, corresponding to 0.27 (95% CI 0.23–0.31) and 0.26 (95% CI 0.23–0.30), respectively. Among 497 permanent quadrats with valid observations in both years, pellet occurrence did not differ (exact McNemar test, p = 1.000).
Figure 3.
Ptarmigan pellet occurrence in permanent 50 × 50 cm quadrats at Erkuta and Sabetta in 2024 and 2025. Open circles and squares show the proportion of checked quadrats containing ptarmigan pellets; error bars show 95% Clopper–Pearson confidence intervals. Sample sizes were 500 and 572 quadrats at Erkuta in 2024 and 2025, respectively, and 284 and 288 quadrats at Sabetta in 2024 and 2025, respectively. Open circles indicate 2024 and open squares indicate 2025.
At Sabetta, pellets were recorded in 17/284 assessable quadrats in 2024 and 10/288 in 2025, corresponding to 0.06 (95% CI 0.03–0.09) and 0.03 (95% CI 0.02–0.06). Among 284 permanent quadrats with valid observations in both years, pellet occurrence did not differ significantly (exact McNemar test, p = 0.230). Thus, neither standardized pellet index indicated higher relative winter–spring ptarmigan occurrence in 2025.
3.6. Spring Temperature and Snow Conditions
Spring conditions at Erkuta differed markedly between years (Table 3; Figure 2). The main snowmelt transition began on 29 May in 2024 and 16 May in 2025 and ended on 7 June and 27 May, respectively. Daily mean air temperature shifted above 0 °C on 20 June in 2024 and 28 May in 2025.
Table 3.
Spring temperature conditions at the Erkuta field site, 2024–2025.
During 15 May–15 June, daily mean temperature was below 0 °C on 21 days in 2024 and 10 days in 2025; daily minimum temperature was below 0 °C on 28 and 17 days, respectively. Positive degree-days were 26.4 in 2024 and 97.8 in 2025.
4. Discussion
Across the three breeding areas, occupancy did not differ between years (35/66 in 2024 vs. 40/69 in 2025; p = 0.606). The proportion of occupied territories with a confirmed nesting attempt increased from 18/35 to 30/40, although not significantly (p = 0.053), whereas hatching success and apparent nesting success among attempts with known outcomes were significantly higher in 2025 (p = 0.003 and p = 0.007, respectively). Thus, the principal interannual contrast arose after territory occupation, showing that relatively stable occupancy can mask marked differences in progression through subsequent reproductive stages [7,8,9].
The reproductive contrast coincided with markedly different spring conditions. At Erkuta, the main snowmelt transition began 13 days earlier and ended 11 days earlier in 2025, daily mean temperature shifted above 0 °C 23 days earlier, and positive degree-days during 15 May–15 June were almost four times higher. This period overlapped incubation and early hatching at many nests. Previous studies indicate that severe weather can affect early Gyrfalcon survival and that snow effects may vary with reproductive stage and prey conditions [6,13,17]. Our observations show a direct nest-scale pathway: at several bridge nests, eggs were laid in snow or ice accumulated within raven-built stick nests, sometimes within snow layers up to approximately 30 cm deep above the underlying nest structure. Incubation depressions and hardened or melted snow around the eggs indicated attempted incubation, showing that a structurally intact nest could remain functionally unsuitable as a dry incubation site. Such attempts were recorded four times in 2024 and once in 2025.
The permanent-quadrat data showed no statistically detectable interannual difference in ptarmigan pellet occurrence at either monitoring site. This result is relevant because ptarmigan are the dominant early-season prey of Gyrfalcons and can influence laying decisions and reproductive performance [12,28,29]. However, pellet occurrence is an indirect index of relative winter–spring occurrence, not a direct estimate of density or short-term prey accessibility around individual territories. The paired results therefore support broadly comparable regional ptarmigan occurrence between years without demonstrating equal local prey availability.
Survey timing differed among breeding areas and requires explicit caution. Schuchya was visited from 15 June to 3 August, so attempts that failed before the first visit were more likely to be missed than on bridges and in the Polar Urals, where surveys covered laying or incubation. However, the interannual difference in hatching success remained significant when Schuchya was excluded (2/10 vs. 14/17; p = 0.003), and the difference in apparent nesting success became stronger (0/8 vs. 13/17; p < 0.001). Thus, Schuchya did not generate the principal interannual pattern. It remains informative for occupied territories, detected attempts, phenology, and later-stage outcomes, but its absolute success estimates and comparisons among substrate groups should not be interpreted as directly equivalent to those from the earlier-visited areas.
Our data most directly support a nest-site mechanism, but they do not identify all pathways through which spring conditions may affect reproduction. Persistent snow or ice was directly observed at failed bridge attempts and can prevent formation of a dry incubation cup. Adult condition, hunting efficiency, and accessibility of adult ptarmigan during courtship and incubation remain plausible complementary mechanisms [6,12], but none were measured directly. Current-year ptarmigan young appear too late to explain Gyrfalcon occupancy, egg laying, or early hatching in the same spring, although they may influence food supply and juvenile survival later in summer. We therefore distinguish the mechanism supported by direct nest observations from hypotheses concerning adult energetics, prey accessibility, and phenological synchrony. Weather and food should be treated as interacting drivers rather than mutually exclusive explanations.
The present design cannot rank tree, rock, bridge, and artificial nests by resilience to late snow. Exposure, nest architecture, sample size, and survey timing differed within and among substrate groups, and snow conditions were not measured systematically at every nest. The coexistence of several nesting substrates may nevertheless provide spatial heterogeneity in exposure across Yamal. Artificial structures should be evaluated experimentally rather than assumed to be protective; designs would need both to limit snow accumulation and to retain nesting material under strong winds [21]. Continued monitoring should therefore focus on nest-specific condition and outcome rather than assigning a general advantage to any substrate category.
These results also caution against equating Arctic warming with uniformly improved breeding conditions. Earlier snowmelt may benefit an early-breeding raptor in some years, while interannual variability in snow accumulation, thaw–refreeze events, and spring snowstorms may still produce poor conditions during laying or incubation [1,3,30]. Repeated thaw and refreezing could create persistent ice on exposed nests, but this mechanism was not measured here and remains a hypothesis. Future monitoring should combine early and late nest checks, standardized recording of snow or ice at individual nests, local temperature loggers where feasible, annual ptarmigan indices, and, where useful, satellite-derived snow-cover data in regions with sparse ground-station coverage. With longer time series, these complementary data could be used to model the relative contributions of weather, prey, and substrate to each reproductive stage.
The results should nevertheless be interpreted in light of several limitations. The study compares only two breeding seasons and therefore cannot separate spring conditions from every unmeasured annual factor, including adult condition, disturbance, predation, or disease. Erkuta was the closest available continuous high-resolution regional station but cannot represent snow depth, wind exposure, solar radiation, or microclimate at every nest. Pellet occurrence does not measure territory-specific prey density, and some hatching and later outcomes remained unresolved. Apparent nesting success was therefore calculated only among attempts with known outcomes and may be biased in either direction. Moreover, field campaigns in these remote Arctic areas require costly specialized transport and are planned well before spring conditions are known, so the unusually late 2024 breeding season could not simply be accommodated by shifting all follow-up visits later. Despite these limitations, several lines of evidence converged: occupancy remained stable, hatching and apparent nesting success differed significantly between years, these differences persisted in the subset of territories surveyed during laying or incubation, regional ptarmigan pellet-occurrence indices did not increase in 2025, and snow- or ice-associated failures were observed directly. Together, these observations identify an interannual association between spring conditions and breeding performance but do not establish a causal weather effect.
5. Conclusions
Across the two breeding seasons, Gyrfalcon nesting-territory occupancy remained similar, whereas hatching success and apparent nesting success among attempts with known outcomes were significantly higher in 2025. Both differences remained significant in the subset of territories where surveys covered laying or incubation. The reproductive contrast coincided with earlier warming and snowmelt and was not accompanied by an increase in either regional ptarmigan pellet-occurrence index. Direct observations of Gyrfalcon eggs laid in snow or ice accumulated within raven-built bridge nests illustrated how persistent spring snow can make an existing nest functionally unsuitable. Together, these observations identify an association between spring conditions and breeding performance rather than demonstrating a causal weather effect, and show why spring conditions, prey, and functional nest-site availability should be evaluated together in Gyrfalcon monitoring and conservation.
Author Contributions
Conceptualization, A.A.S.; methodology, A.A.S., N.A.S., V.A.S. and I.A.F.; validation, A.A.S. and I.A.F.; formal analysis, A.A.S. and I.A.F.; investigation, A.A.S., N.A.S., V.A.S., I.A.F., S.A.M. and A.A.E.; resources, A.A.S., V.A.S. and S.A.M.; data curation, A.A.S., N.A.S., V.A.S., I.A.F. and S.A.M.; writing—original draft preparation, N.A.S.; writing—review and editing, A.A.S., N.A.S., V.A.S., I.A.F., S.A.M. and A.A.E.; visualization, A.A.S. and I.A.F.; supervision, A.A.S.; project administration, A.A.S.; funding acquisition, A.A.S., V.A.S. and I.A.F. All authors have read and agreed to the published version of the manuscript.
Funding
This study was supported by Russian Science Foundation, grant no. 24-44-00094.
Institutional Review Board Statement
Ethical review and approval were waived for this study because it was based on non-invasive field observations, nest checks, photography, UAV inspections, and camera-trap monitoring. No Gyrfalcons were captured, handled, marked, or experimentally manipulated.
Informed Consent Statement
Not applicable.
Data Availability Statement
The original contributions presented in this study are included in the article. Further inquiries can be directed to the corresponding author. Exact nest and territory coordinates are not publicly released to protect breeding sites of a sensitive raptor species.
Acknowledgments
We sincerely thank Vyacheslav Osokin for his help in surveys of the Polar Ural foothills and Valeriy Fedorovich Rudkovskiy for co-leading surveys of the railway bridges.
Conflicts of Interest
The authors declare no conflicts of interest.
References
- Post, E.; Forchhammer, M.C.; Bret-Harte, M.S.; Callaghan, T.V.; Christensen, T.R.; Elberling, B.; Fox, A.D.; Gilg, O.; Hik, D.S.; Høye, T.T.; et al. Ecological dynamics across the Arctic associated with recent climate change. Science 2009, 325, 1355–1358. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gilg, O.; Kovacs, K.M.; Aars, J.; Fort, J.; Gauthier, G.; Grémillet, D.; Ims, R.A.; Meltofte, H.; Moreau, J.; Post, E.; et al. Climate change and the ecology and evolution of Arctic vertebrates. Ann. N. Y. Acad. Sci. 2012, 1249, 166–190. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- IPCC. Climate Change 2023: Synthesis Report. Contribution of Working Groups I, II and III to the Sixth Assessment Report of the Intergovernmental Panel on Climate Change; Core Writing Team, Lee, H., Romero, J., Eds.; IPCC: Geneva, Switzerland, 2023. [Google Scholar] [CrossRef] [Scilit]
- Newton, I. Population limitation in birds of prey: A comparative approach. In Bird Population Studies: Relevance to Conservation and Management; Perrins, C.M., Lebreton, J.-D., Hirons, G.J.M., Eds.; Oxford University Press: Oxford, UK, 1991; pp. 3–21. [Google Scholar]
- Anctil, A.; Franke, A.; Bêty, J. Heavy rainfall increases nestling mortality of an arctic top predator: Experimental evidence and long-term trend in Peregrine Falcons. Oecologia 2014, 174, 1033–1043. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Franke, A. Priorities for Gyrfalcon research: Food, weather, and phenology in a changing climate. In Applied Raptor Ecology: Essentials from Gyrfalcon Research; Anderson, D.L., McClure, C.J.W., Franke, A., Eds.; The Peregrine Fund: Boise, ID, USA, 2017; pp. 11–32. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Steenhof, K.; Newton, I. Assessing nesting success and productivity. In Raptor Research and Management Techniques; Bird, D.M., Bildstein, K.L., Eds.; Hancock House: Blaine, WA, USA, 2007; pp. 181–192. [Google Scholar]
- Franke, A.; McIntyre, C.L.; Steenhof, K. Terminology. In Applied Raptor Ecology: Essentials from Gyrfalcon Research; Anderson, D.L., McClure, C.J.W., Franke, A., Eds.; The Peregrine Fund: Boise, ID, USA, 2017; pp. 33–42. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Steenhof, K.; Kochert, M.N.; McIntyre, C.L.; Brown, J.L. Coming to terms about describing Golden Eagle reproduction. J. Raptor Res. 2017, 51, 378–390. [Google Scholar] [CrossRef] [Scilit]
- Cade, T.J. Biological traits of the Gyrfalcon (Falco rusticolus) in relation to climate change. In Gyrfalcons and Ptarmigan in a Changing World, Vol. I; Watson, R.T., Cade, T.J., Fuller, M., Hunt, G., Potapov, E., Eds.; The Peregrine Fund: Boise, ID, USA, 2011; pp. 33–44. [Google Scholar] [CrossRef] [Scilit]
- Franke, A.; Falk, K.; Hawkshaw, K.; Ambrose, S.; Anderson, D.L.; Bente, P.J.; Booms, T.; Burnham, K.K.; Carrière, S.; Ekenstedt, J.; et al. Status and trends of circumpolar Peregrine Falcon and Gyrfalcon populations. Ambio 2020, 49, 762–783. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nielsen, Ó.K.; Cade, T.J. Gyrfalcon and ptarmigan predator-prey relationship. In Applied Raptor Ecology: Essentials from Gyrfalcon Research; Anderson, D.L., McClure, C.J.W., Franke, A., Eds.; The Peregrine Fund: Boise, ID, USA, 2017; pp. 43–74. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Slettenhaar, A.J.; Østnes, J.E.; Moen, B.C.; Kroglund, R.T.; Nygård, T.; Nilsen, E.B. A picky predator and its prey: How snow conditions and ptarmigan abundance impact Gyrfalcon feeding behaviour and breeding success. Ecol. Evol. 2025, 15, e71228. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gustafson, M.; McCabe, J.D.; Rolek, B.W.; Booms, T.L.; Henderson, M.T.; Dunn, L.; Anderson, D.L.; Cruz, J. Gyrfalcon prey abundance and their habitat associations in a changing Arctic. Ecol. Evol. 2025, 15, e70763. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kleiven, E.F.; Johansen, K.; Ims, R.A.; Soininen, E.M.; Oksanen, L.; Oksanen, T.; Jacobsen, K.-O.; Østlyngen, A. A specialist predator in a food web with cyclic alternative prey: The Gyrfalcon–ptarmigan case revisited. J. Anim. Ecol. 2025, 94, 1193–1203. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cade, T.J. Ecology of the Peregrine and Gyrfalcon populations in Alaska. Univ. Calif. Publ. Zool. 1960, 63, 151–290. [Google Scholar]
- Poole, K.G.; Bromley, R.G. Natural history of the Gyrfalcon in the central Canadian Arctic. Arctic 1988, 41, 31–38. [Google Scholar] [CrossRef] [Scilit]
- Beardsell, A.; Gauthier, G.; Therrien, J.-F.; Bêty, J. Nest site characteristics, patterns of nest reuse, and reproductive output in an Arctic-nesting raptor, the Rough-legged Hawk. Auk 2016, 133, 718–732. [Google Scholar] [CrossRef] [Scilit]
- Forbes, B.C. Land use and climate change on the Yamal Peninsula of north-west Siberia: Some ecological and socio-economic implications. Polar Res. 1999, 18, 367–373. [Google Scholar] [CrossRef] [Scilit]
- Walker, D.A.; Leibman, M.O.; Epstein, H.E.; Forbes, B.C.; Bhatt, U.S.; Raynolds, M.K.; Comiso, J.C.; Gubarkov, A.A.; Khomutov, A.V.; Jia, G.J.; et al. Spatial and temporal patterns of greenness on the Yamal Peninsula, Russia: Interactions of ecological and social factors affecting the Arctic normalized difference vegetation index. Environ. Res. Lett. 2009, 4, 045004. [Google Scholar] [CrossRef] [Scilit]
- Mechnikova, S.A.; Fufachev, I.A.; Kitel, D.A.; Yesergepov, A.A.; Kudryavtsev, N.V.; Bogomolov, D.V.; Kostenko, A.V.; Zakharova, N.Y.; Mechnikova, K.T.; Sakharova, T.V.; et al. A long-term conservation initiative: Artificial nests for Falco rusticolus (Falconidae) in Southern Yamal, North-West Siberia. Nat. Conserv. Res. 2026, 11, 1–9. [Google Scholar] [CrossRef] [Scilit]
- Sokolov, A.A.; Fufachev, I.A.; Sokolov, V.A.; Sokolova, N.A.; Golovatin, M.G.; Dixon, A. Gyrfalcons in a man-made landscape of the Yamal Peninsula. Fauna Ural. I Sib. 2017, 2, 180–185, (In Russian with English Summary). [Google Scholar]
- Matveeva, T.; Sidorchuk, A. Modelling of surface runoff on the Yamal Peninsula, Russia, using ERA5 reanalysis. Water 2020, 12, 2099. [Google Scholar] [CrossRef] [Scilit]
- Ardelean, F.; Onaca, A.; Chețan, M.-A.; Dornik, A.; Georgievski, G.; Hagemann, S.; Timofte, F.; Berzescu, O. Assessment of spatio-temporal landscape changes from VHR images in three different permafrost areas in the western Russian Arctic. Remote Sens. 2020, 12, 3999. [Google Scholar] [CrossRef] [Scilit]
- Anderson, D.L.; Burnham, K.K.; Nielsen, Ó.K.; Robinson, B.W. A photographic and morphometric guide to aging Gyrfalcon nestlings. In Applied Raptor Ecology: Essentials from Gyrfalcon Research; Anderson, D.L., McClure, C.J.W., Franke, A., Eds.; The Peregrine Fund: Boise, ID, USA, 2017; pp. 265–282. [Google Scholar] [CrossRef] [Scilit][Green Version]
- Ehrich, D.; Henden, J.-A.; Ims, R.A.; Doronina, L.O.; Killengren, S.T.; Lecomte, N.; Pokrovsky, I.G.; Skogstad, G.; Sokolov, A.A.; Sokolov, V.A.; et al. The importance of willow thickets for ptarmigan and hares in shrub tundra: The more the better? Oecologia 2012, 168, 141–151. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Agresti, A. Categorical Data Analysis, 3rd ed.; Wiley: Hoboken, NJ, USA, 2013. [Google Scholar]
- Barichello, N.; Mossop, D.H. The overwhelming influence of ptarmigan abundance on Gyrfalcon reproductive success in the central Yukon, Canada. In Gyrfalcons and Ptarmigan in a Changing World, Vol. I; Watson, R.T., Cade, T.J., Fuller, M., Hunt, G., Potapov, E., Eds.; The Peregrine Fund: Boise, ID, USA, 2011; pp. 307–322. [Google Scholar] [CrossRef] [Scilit]
- Nielsen, Ó.K. Gyrfalcon predation on ptarmigan: Numerical and functional responses. J. Anim. Ecol. 1999, 68, 1034–1050. [Google Scholar] [CrossRef] [Scilit]
- Sokolov, A.A.; Sokolova, N.A.; Ims, R.A.; Brucker, L.; Ehrich, D. Emergent rainy winter warm spells may promote boreal predator expansion into the Arctic. Arctic 2016, 69, 121–129. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.