Article

Substrate-Dependent Responses of Radish to Anaerobically Fermented Furcellaria lumbricalis Biostimulant Under Reduced Mineral Fertilization

1
Faculty of Agriculture and Food Technology, Latvia University of Life Sciences and Technologies, LV 3004 Jelgava, Latvia
2
Faculty of Economics and Social Development, Latvia University of Life Sciences and Technologies, LV 3001 Jelgava, Latvia
3
Liepaja Academy, Riga Technical University, LV 3401 Liepaja, Latvia
*
Authors to whom correspondence should be addressed.
These authors contributed equally to this work.
Agronomy 2026, 16(8), 837; https://doi.org/10.3390/agronomy16080837
Submission received: 14 March 2026 / Revised: 16 April 2026 / Accepted: 18 April 2026 / Published: 21 April 2026
(This article belongs to the Special Issue Sustainable Strategies for Enhancing Soil Health and Food Quality)

Abstract

Modern agriculture is increasingly reliant on imported fertilizers and subject to price volatility, compounded by environmental pressures arising from the overuse of synthetic fertilizers. This study assessed the impact of Furcellaria lumbricalis algal biostimulant, produced by anaerobic fermentation, on dry matter yield and plant development indicators of garden radish (Raphanus raphanistrum subsp. sativus) in five soil substrate types. Biostimulant doses aimed at reducing mineral fertilizer application to 75% of the full rate while maintaining or improving yield were evaluated; yet no statistically significant effect on dry matter yield was observed, and the hypothesis was therefore not statistically confirmed. The experiment included five substrate types (sandy clay, sandy clay with organic matter, sand, sand with organic matter, and peat) and six fertilizer/biostimulant treatments, including 75% mineral fertilizer combined with 3%, 6%, and 12% algal biostimulant concentrations. Linear mixed models showed that substrate type (F = 19.58; p < 0.001) and fertilizer variant (F = 5.00; p < 0.001) had statistically significant effects on total dry matter yield, but their interaction was not statistically significant. All 75% and 100% mineral fertilizer variants with and without biostimulant produced statistically significantly higher yields than the unfertilized control (p = 0.0016–0.0337). The leaf development indicator (AtLeaf) index was statistically significantly higher in all biostimulant variants compared to the unfertilized control. Principal component analysis (PCA) and redundancy analysis (RDA) demonstrated that substrate type determines the primary structure of the substrate–plant system, while biostimulant effects were expressed as modulation of existing processes within the substrates. The results indicate substrate-specific responses to Baltic Sea algal Furcellaria lumbricalis digestate with statistically significant effect observed only in peat, consistent with previous findings, while no significant effects were detected in other substrates. Although the effects of the biostimulant on dry matter yield were not consistently statistically significant, the observed trends in plant development indicators and substrate–plant system responses suggest that Furcellaria lumbricalis digestate may have potential as a nutrient recycling component within a circular bioeconomy framework.

1. Introduction

Global agriculture faces strategic risks compounded by geopolitical conflicts and their impact on fertilizer supply chains [1,2,3,4,5]. Russia’s invasion of Ukraine has significantly disrupted the fertilizer market, as Russia and Belarus together account for a substantial share of global nitrogen and potassium fertilizer exports, thus causing rapid price increases and supply volatility. The rise in the fertilizer price index and the increase in phosphate prices in recent years, with nitrogen fertilizer prices rising by 43% and phosphate prices by 28% between 2022 and 2024 [1,3,5], underscore the need for resource-efficient alternatives to synthetic fertilizers.
Plant biostimulants have gained increasing attention as a method for enhancing resource efficiency. These products stimulate plant physiological processes independently of their nutrient content, leading to improved nutrient use efficiency (NUE), greater tolerance to abiotic stresses and enhanced product quality [6,7,8,9,10]. Elevated fertilizer prices increase the economic incentive for adopting biostimulants, which can allow lower fertilizer doses while maintaining agronomic performance. Prior research has demonstrated that seaweed extracts can markedly promote plant growth and productivity by influencing root development, photosynthesis, antioxidative defenses and the rhizosphere microbiome [7,11,12,13]. Meta-analyses indicate that biostimulants increase crop yields by 15–17% on average, with seaweed extracts producing even greater yield increases and improving nutrient efficiency by 16–38% in some studies [14,15,16].
Recent advances in metabolomics and transcriptomics have revealed that seaweed-based biostimulants act through multiple interconnected pathways, including phytohormonal regulation, signal transduction via polysaccharide-induced priming and activation of stress-response genes, collectively enhancing plant resilience and yield [11,12,13,17]. In addition to their direct effects on plant physiology, seaweed-derived biostimulants have been reported to influence soil biological activity and microbial processes. Polysaccharides such as carrageenans may act as substrates for beneficial microorganisms, supporting nutrient-cycling processes such as nitrogen transformation and phosphorus mobilization [13,16,18]. However, these effects are often indirect and dependent on substrate properties and environmental conditions. Additionally, Kappaphycus-based biostimulants have been shown to substantially modify the rhizosphere microbiome by increasing populations of beneficial microorganisms, potentially enhancing nitrogen fixation and phosphorus solubilization and producing synergistic effects beyond the biostimulant’s nutrient content.
Most research on seaweed biostimulants has focused on tropical and subtropical species such as Kappaphycus, Gracilaria, and Sargassum. In contrast, studies on temperate-region seaweeds, including those from the Baltic Sea, remain limited [13,14,15,16,17]. Furthermore, there is a lack of systematic analysis on how soil properties, particularly organic matter content and pH, affect biostimulant efficacy when mineral fertilizer use is reduced [10,19,20,21,22,23,24,25]. The available literature presents conflicting recommendations on optimal dosage, with effective concentrations ranging from 0.1% to 12% (v/v), depending on the product, crop and environmental conditions [11,14,15,16,25,26,27].
The use of digestate from anaerobic fermentation is recognized as a key opportunity for the circular bioeconomy, simultaneously yielding renewable energy (biogas) and nutrient-rich by-products with the potential to partially replace synthetic fertilizers [19,20,21,22,23,28,29,30,31,32]. The circular bioeconomy framework emphasizes closing nutrient cycles by converting organic waste into high-value products and reducing reliance on mineral resource extraction [31,32,33]. Seaweed biomass is of particular interest in this context since it enables a combination of coastal management, biogas production, and digestate use, as highlighted by several Life Cycle Assessment (LCA) studies in northern Europe [34,35,36,37].
Furcellaria lumbricalis, a Baltic red seaweed, contains high levels of dry matter, active metabolites, and low pollutant concentrations, making it suitable for agricultural applications. Previous studies have integrated Furcellaria lumbricalis into coastal biomass valorization frameworks [34,35,36,37,38,39]. Studies have demonstrated that anaerobically fermented digestate (3–6%) from this seaweed species increases leafy vegetable biomass, reduces mineral fertilizer inputs while maintaining or improving yields, and stimulates soil microbial activity. Polysaccharides such as carrageenans and other bioactive compounds present in Furcellaria lumbricalis digestate may act as selective substrates for beneficial microorganisms, potentially supporting microbial processes related to nitrogen cycling and phosphorus mobilization [13,16,18].
This study was conducted to evaluate the effects of anaerobically fermented Furcellaria lumbricalis digestate on radish growth across different soil substrates and its potential to reduce mineral fertilization application. Dry matter yield and plant development indicators were assessed across five substrate types under reduced (75%) mineral fertilization combined with different biostimulant doses. It was hypothesized that Furcellaria lumbricalis digestate may contribute to reducing mineral input fertilizers while maintaining yield and enhancing plant development, depending on substrate type. The study was conducted as a controlled pot experiment with multiple substrate and treatment combinations, followed by multivariate statistical analysis.

2. Materials and Methods

This study is the first to systematically evaluate the effects of Furcellaria lumbricalis digestate from Baltic Sea red algae on garden radish grown in diverse mineral and organic substrates under a 75%-of-standard mineral fertilizer regime, integrating agronomic, soil and economic indicators into a unified analysis. The study was conducted in sequential stages, from algal biomass collection and digestate production to pot experiments across different soil substrates and multivariate statistical analysis, as illustrated in Figure 1.

2.1. Obtaining Algae Biostimulant

The algal biostimulant was produced by anaerobic fermentation, during which the digestate—comprising a solid and a liquid fraction—was obtained alongside biogas. This study used the liquid fraction of the digestate because it contains readily available macro- and trace elements (nitrogen, potassium and trace minerals), organic acids and microbial metabolites that stimulate plant growth and improve soil biological activity [28,29,30]. The digestate is enriched with polysaccharides and mineral salts characteristic of Furcellaria lumbricalis biomass, and has been shown to improve plants’ resistance to abiotic stress, increase nutrient uptake and promote root system development [44,45]. The raw material was the red seaweed Furcellaria lumbricalis washed ashore after autumn storms and was collected from the beach without mechanical disturbance to underwater algal populations, thereby ensuring environmentally responsible biomass procurement. The harvested biomass was rinsed with fresh water prior to fermentation to remove sand and mechanical impurities, then naturally dried and stored until used in the fermentation process. Fermentation was performed in a sealed, thermally insulated 30 L polymer reactor (RTU, Liepaja, Latvia) equipped with a mixer, a biogas drainage and analysis system, a cable heating element, and temperature control devices. Mesophilic conditions (37 °C) were maintained with an accuracy of ±0.5 °C to ensure stable process conditions. Where necessary, pH was adjusted by adding diluted sodium hydroxide (NaOH). Sensor hardware and a Raspberry Pi 4B-based data logging system (Raspberry Pi Foundation, Cambridge, UK) were integrated into the reactor. The process was monitored using (1) Dallas DS18B20 digital temperature sensors (Maxim Integrated, San Jose, CA, USA), (2) an MQ4 methane concentration sensor (Zhengzhou Winsen Electronics Technology Co., Ltd., Zhengzhou, China), (3) an ATO MF5706 gas flow meter (ATO Inc., Chengdu, China), and (4) a GETI PM001 electricity meter (distributed by TIPA, spol. s r.o., Opava, Czech Republic). After anaerobic fermentation, the digestate was mechanically separated using a 2 × 2 mm sieve. The chemical composition of the digestate obtained from anaerobic digestion of Furcellaria lumbricalis (expressed on a fresh weight basis) was as follows: pH (KCl) 5.4, dry matter content 2.07%, total nitrogen (N) 0.10%, total phosphorus (P2O5) 0.03%, and total potassium (K2O) 0.24%. These parameters represent the main physicochemical characteristics of the undiluted digestate used in the experiment. The filtered digestate was stored in closed containers at room temperature until use in subsequent trials.

2.2. Experiment Setup and Substrate Characterization

A trial of vegetation containers in covered areas at the Institute of Soil and Plant Sciences of Latvia University of Life Sciences and Technologies (hereinafter—LBTU) was established to evaluate the efficiency of biostimulants. Garden radish (Raphanus raphanistrum subsp. sativus) was grown in five substrates: sandy clay (Clay), sandy clay with organic matter (ClayOM), sand (Sand), sand with organic matter (SandOM), and peat (Peat). In addition, there were three control options—no fertilizer in (F0_BIO0), with 100% (F100_BIO0) of mineral fertilizers and 75% full dose (F75_BIO0)—and three options with 75% doses of mineral fertilizers with algae biostimulant at concentrations of 3, 6 and 12% (F75_BIO3, F75_BIO6, F75_BIO12). Characteristics of the biostimulant in naturally wet material: pH KCl 5.4; dry matter content 2.07%; total nitrogen content 0.10%; total phosphorus content as P2O5 0.026%; total potassium content as K2O 0.235%. The combination of each substrate and variant was realized in three independent replicates, with a total of 90 experimental units. Four mineral soil types differing in texture and organic matter content, were selected for the growing substrate, collected on 7 October 2024 in the “Pēterlauki” area of the LBTU training and study farm and neutralized peat substrate (pH 5.0). Samples characterized as silty clay by grading (as determined by the FAO field method) were collected from a long-fallow section of the field (56°30′29.9″ N, 23°41′22.9″ E). The soil’s surface mineral hummus accumulation horizon was used for test variants with elevated organic matter content (ClayOM), while the illuvial horizon below was used for variants with reduced organic matter content (Clay). The sandy substrate was obtained on permanent grassland without intensive agricultural activity (56°42′20.4″ N, 23°47′22.9″ E). In this case, the illuvial soil horizon below the sod layer (SandOM) and the deeper following horizon with lower organic matter content (Sand) were used. After harvesting, the soil was homogenized, stored for a week, then re-homogenized manually and filled into 5 L of vegetation containers. Chemical analyses of mineral substrates were carried out during the waiting period (Table 1).
Table 1 summarizes the main chemical characteristics of the substrates used in the experiment, highlighting a pronounced gradient in organic matter and nutrients, from mineral substrates with insufficient organic matter content and low phosphorus and potassium levels to peat with very high organic matter content, low phosphorus availability and very high potassium content. Such a gradient provides different nutrient availability and buffer capacity conditions, which allow the efficacy of the biostimulant in both nutrient-poor and organic substrates to be assessed, as recommended in other multi-factor digestate and biostimulant studies [46,47].
The following analytical methods were used for all soil samples during the test: the environmental response of the substrate is determined in a 1 M KCl suspension according to the ISO 10390:2005 [40] method in two iterations; the content of mobile phosphorus and potassium is determined by the Egner–Rhiehm (DL) method in three iterations; organic matter content is determined by the Walkley–Black method using GLOSOLAN-SOP-02 (titrimetry and colorimetric method) in three iterations.
Carbamide (46.2% N), single superphosphate (19% P2O5) and potassium sulphate (51% K2O) were used for fertilization. According to the experimental variant and the specified norms of the crop (Table 2), mineral fertilizers were weighed, dissolved, and incorporated into each vegetation container separately, thus ensuring rapid exposure of fertilizers and a uniform distribution of substances throughout the volume of the substrate.
Table 2 presents the N, P2O5, and K2O doses applied in the various treatment variants, reflecting both the full 100% mineral fertilizer norm and the 75% dose scenarios with and without Furcellaria lumbricalis digestate. This design allows direct comparison of whether 75% NPK combined with biostimulant produces similar dry matter yield to the full NPK dose, in line with typical radish fertilization recommendations for the Baltic region.
Soil microbial activity was assessed in all experimental substrates using the cellulose degradation intensity method, following the protocol described in Skapste et al., 2025 [38] without modification.

2.3. Statistical Analysis

Statistical data processing was performed using the R language for statistical computing in RStudio (version 4.5.2). For analysis of total dry matter yield, a linear mixed model was applied, with substrate type and biostimulant variant included as fixed effects and biological replicates as random effects. The statistical significance of fixed effects was assessed using Type III ANOVA with Satterthwaite approximation of degrees of freedom. Model assumptions were verified by analyzing the distribution of residuals and homogeneity of variance; normality of residuals was assessed by the Shapiro–Wilk test. The explained variation in the model was described by calculating marginal and conditional coefficients of determination (R2), characterizing the fixed effects and total explained variation in the model, respectively. As the interaction between substrate type and biostimulant variant was not statistically significant, biostimulant variants were compared with the control using an additive model without an interaction term. Comparisons were made using Dunnett contrasts against the unfertilized control (F0_BIO0). Principal component analysis (PCA) was performed to characterize the structure of soil chemical and biological indicator data, identifying predominant variation gradients and substrate groupings in multidimensional space. Interpretation of principal components was based on variable loadings and the proportion of variation explained. Redundancy analysis (RDA) was used to quantify the contribution of substrate type and biostimulant variant to variation in soil properties, with factor significance tested using 999 permutations. Pearson correlation coefficients were calculated between total dry matter yield and selected soil and plant development indicators. For analysis of the leaf development indicator measured using the atLEAF CHL PLUS chlorophyll meter, FT Green LLC, Wilmington, DE, USA (hereafter referred to as AtLeaf), a linear model was applied including total dry matter yield, substrate type, and biostimulant variant as explanatory variables.

3. Results

3.1. Total Dry Matter Yield

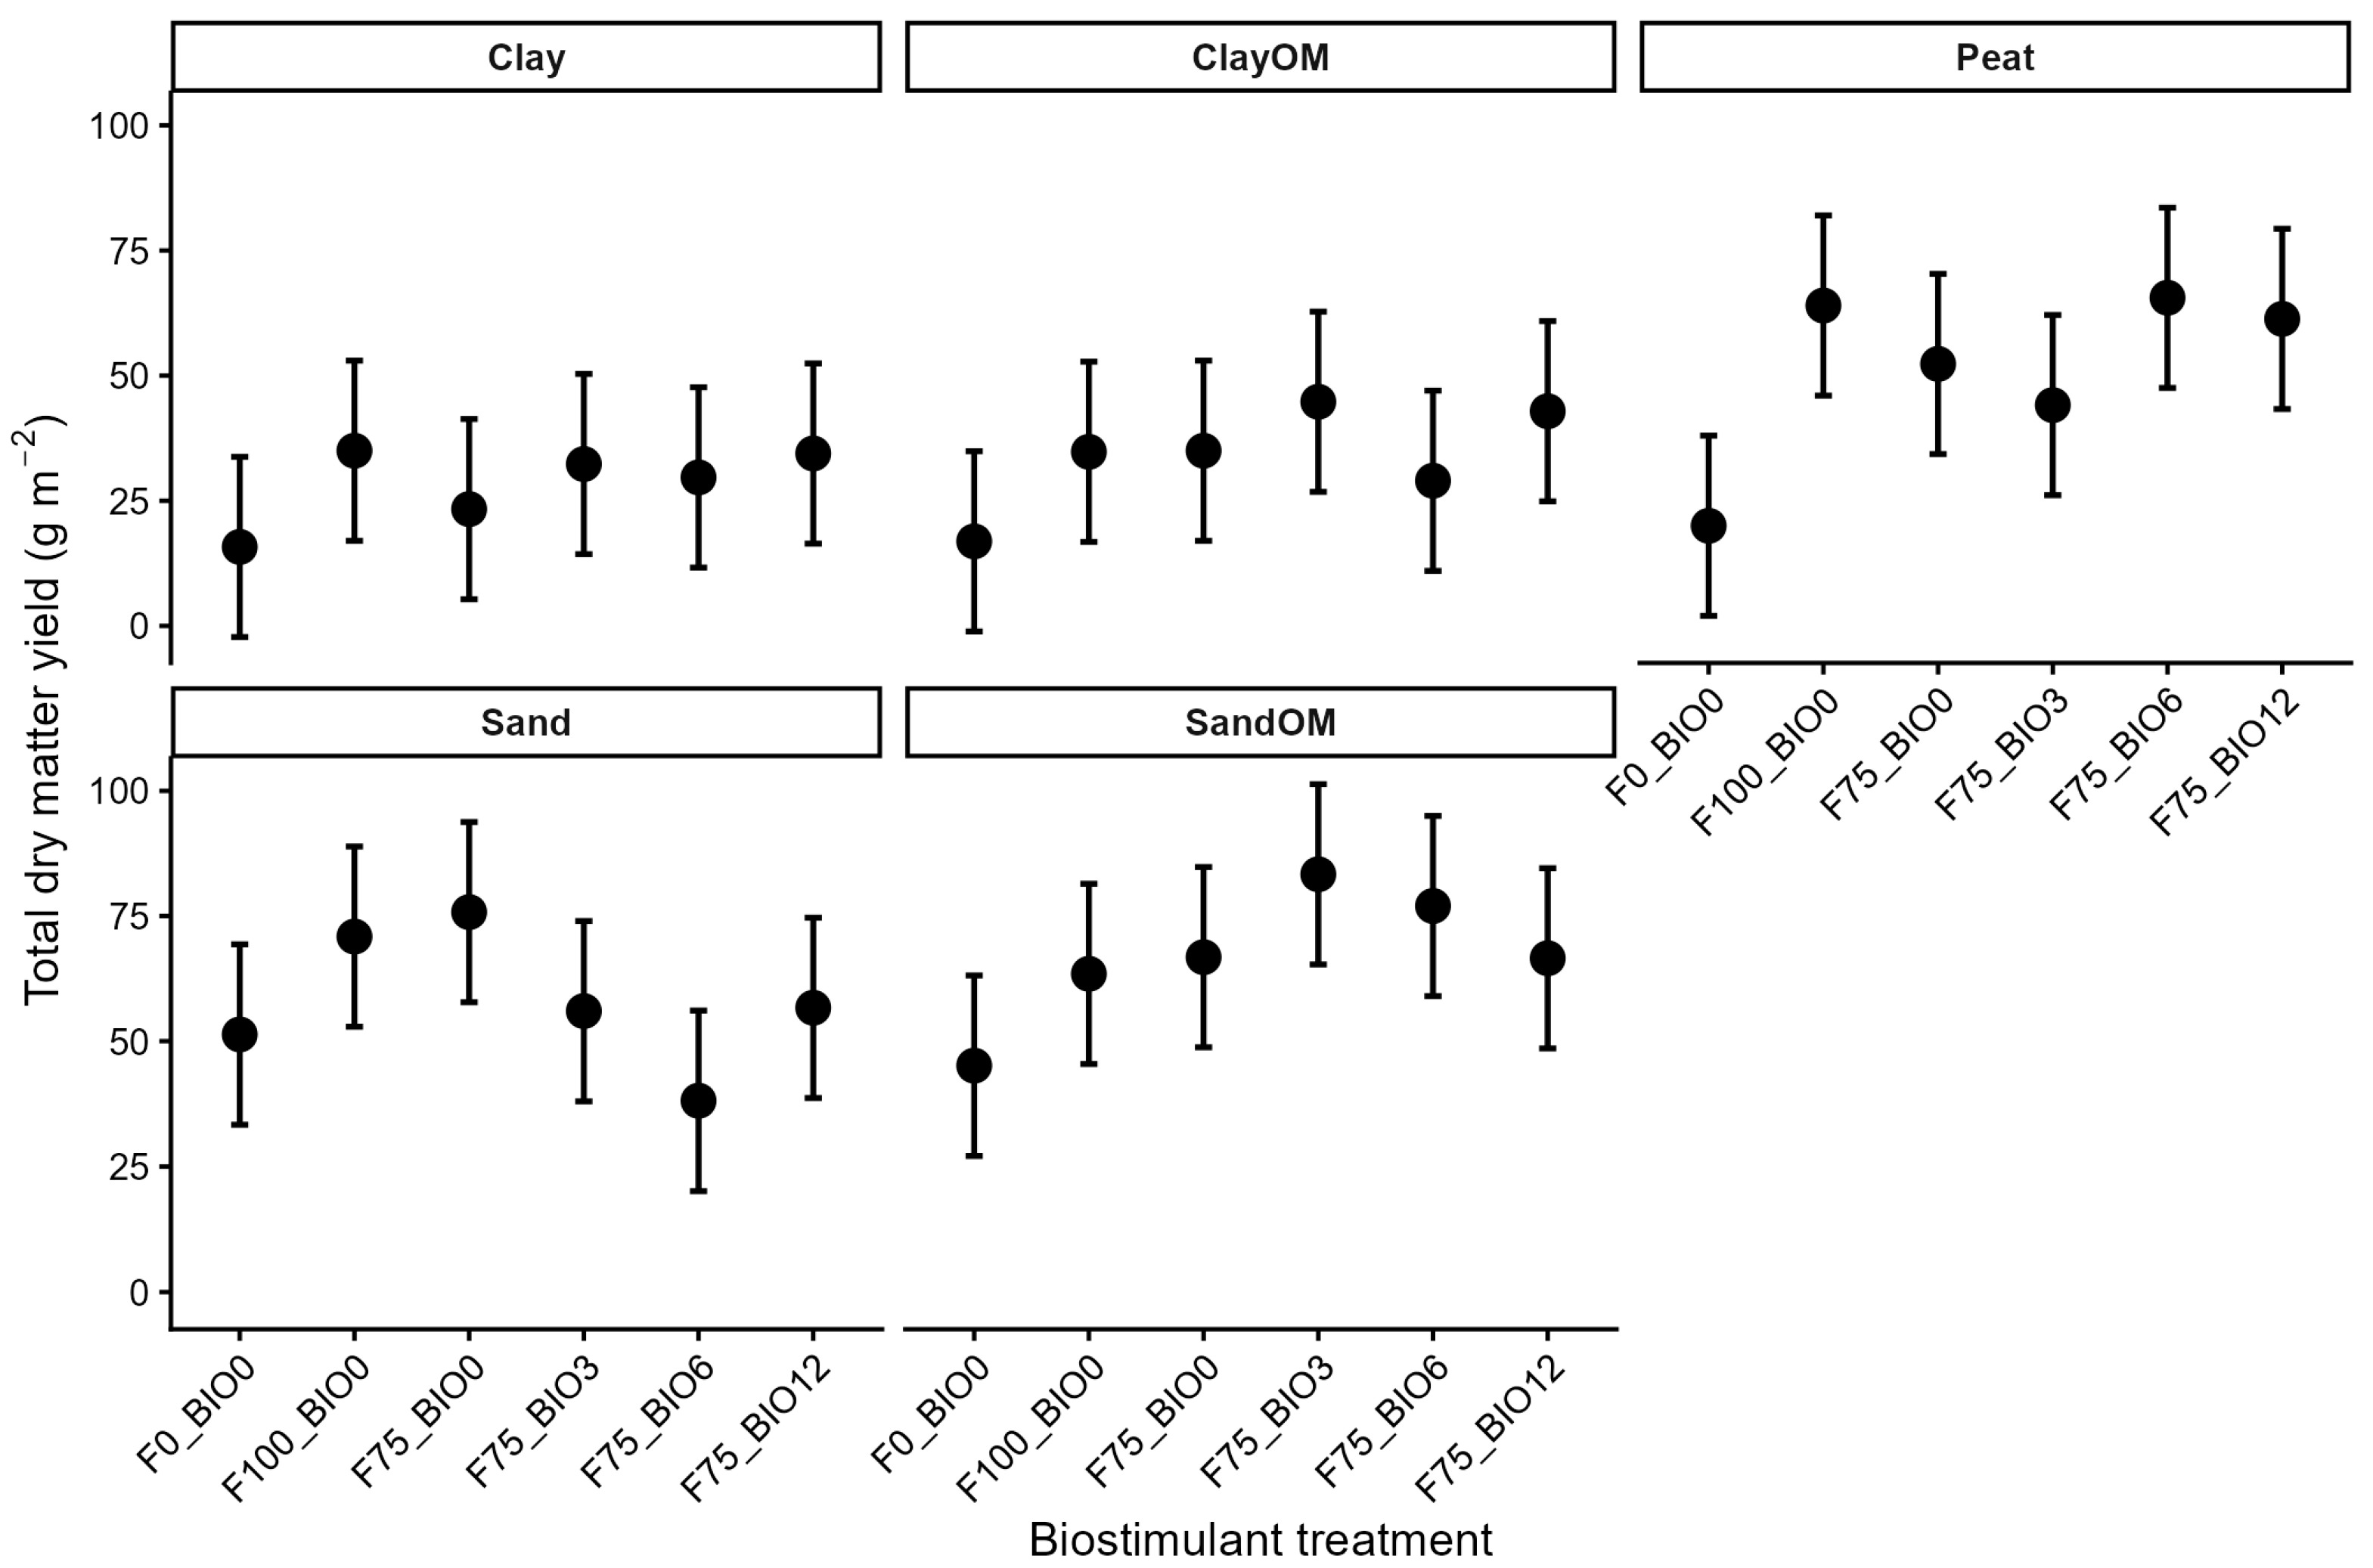
At the 75% mineral fertilizer dose, the effect of the algal biostimulant on total dry matter yield varied by substrate type (Figure 2), as indicated by differences in estimated marginal means across substrates and treatment variants in the linear mixed model. Although biostimulant doses were associated with higher modeled dry matter yield values in individual substrates compared to the F75_BIO0 and F100_BIO0 variants, no statistically significant differences were observed in most pairwise dose comparisons, as demonstrated by 95% overlap in confidence intervals.
The highest modeled dry matter yield values in clay and clay-with-organic matter substrates were observed at the 12% biostimulant dose, reaching levels in the clay substrate that were not statistically different from the full mineral fertilizer variant (F100_BIO0). Similar but less pronounced trends were observed in these substrates at the 3% biostimulant dose.
In the sand substrate, the mixed-model results indicated lower dry matter yield values at biostimulant doses, with the most marked decrease at the 6% dose. In contrast, in sand with organic matter, biostimulant doses were generally associated with higher modeled dry matter yield values than the F75_BIO0 variant, in some cases reaching levels similar to or slightly higher than F100_BIO0.
In the peat substrate, slightly higher modeled dry matter yield values were observed for biostimulant treatment variants compared to F75_BIO0; however, the mixed-model analysis did not reveal statistically significant differences between treatment variants.
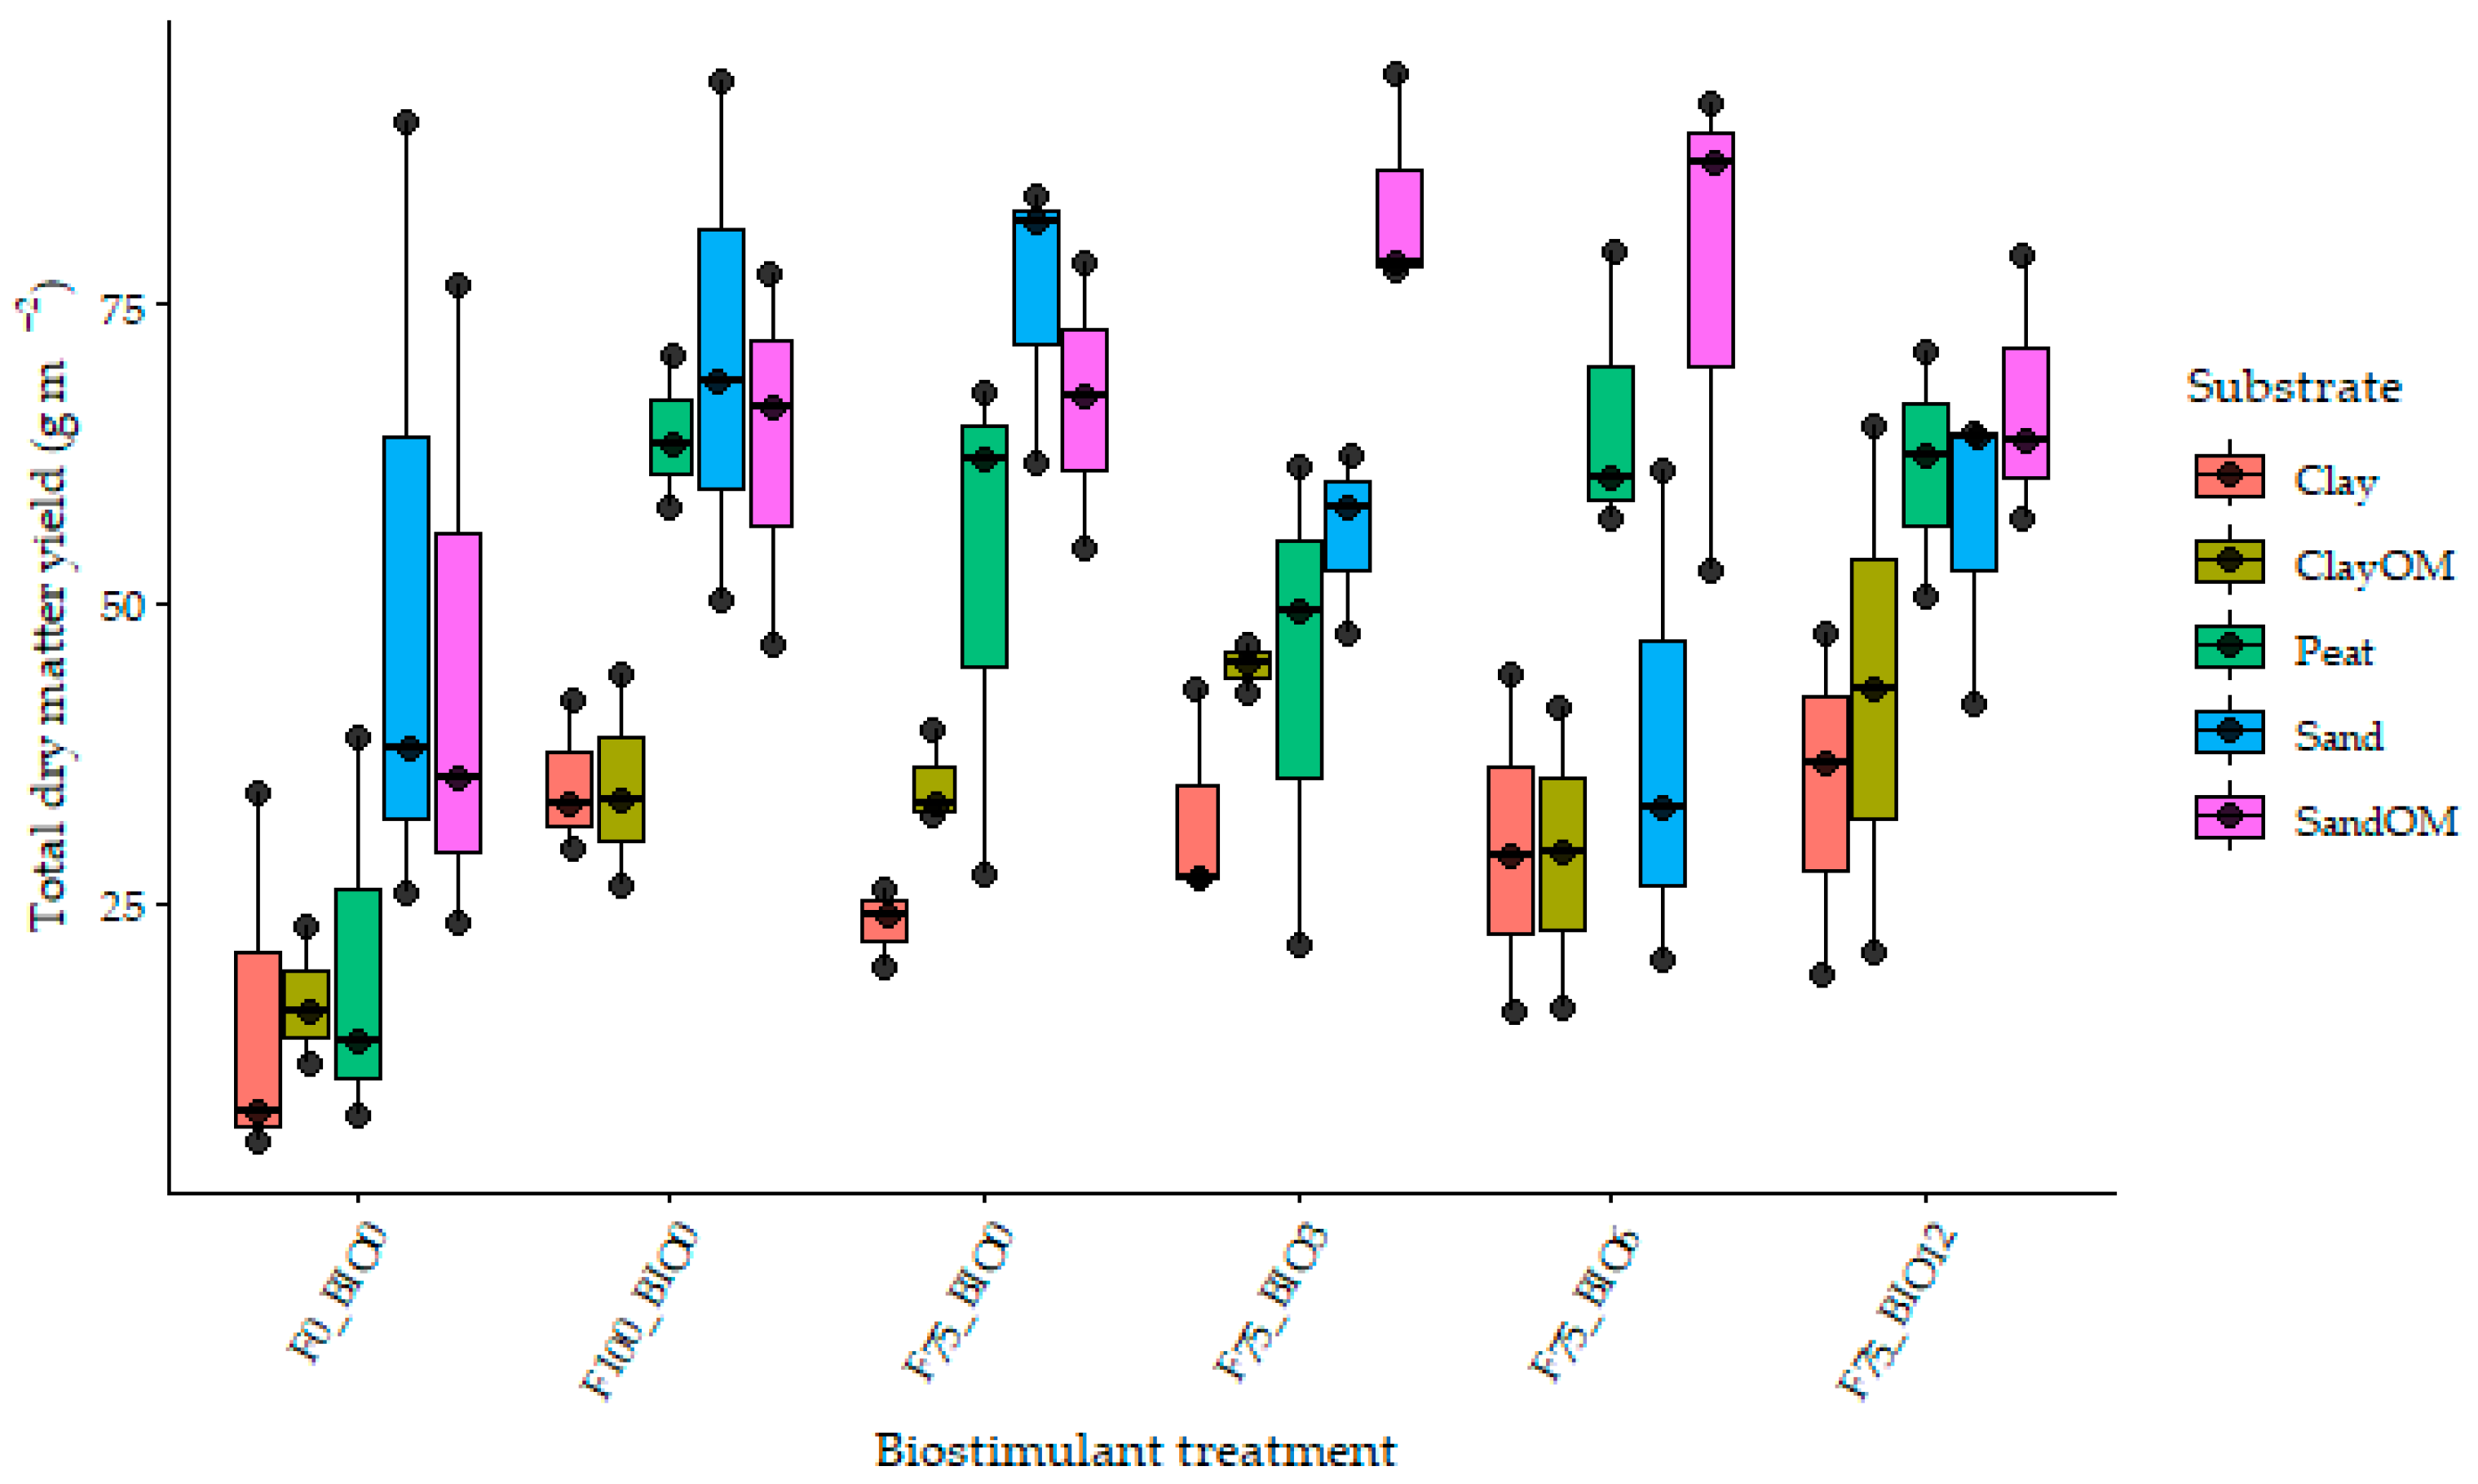
The distribution of individual dry matter yield values across substrates and treatment variants is shown in Figure A1 (Appendix A). The quantitative characterization of dry matter yield distribution across substrates at 75% NPK combined with digestate provides an assessment of dry matter yield patterns across substrate types. In some cases, mean values approached those observed under full mineral fertilizer, particularly in clay and clay-with-organic-matter substrates.

3.2. Impact Assessment of Substrate and Biostimulant

A two-factor ANOVA showed that both substrate type (F(4, 60) = 19.58; p < 0.001) and treatment variant (F(5, 60) = 5.00; p < 0.001) had statistically significant effects on total dry matter yield. Model residuals satisfied the normality assumption (Shapiro–Wilk test, p > 0.05). The interaction between substrate type and treatment variant was not statistically significant (F(20, 60) = 1.27; p = 0.235), indicating that the pattern of treatment effects did not differ significantly across substrate types.
Substrates containing organic matter and peat exhibited greater variation in dry matter yield among biostimulant treatments than mineral substrates; however, statistically significant differences were observed only in peat substrate. The corresponding one-way ANOVA results for each substrate are presented in Table A1 (Appendix A).
In the linear mixed model, the proportion of variance explained by fixed effects (substrate type and biostimulant variant) the marginal R2 was 0.591; the contribution of the random effect (biological replication) was minimal, resulting in a conditional R2 equal to the marginal R2 (0.591). Since the interaction between substrate type and treatment variant was not statistically significant, an additive model without the interaction term was used for further comparison of treatment variants, and Dunnett post-hoc contrasts against the unfertilized control were performed.
Compared with the unfertilized control (F0_BIO0), all fertilized treatments (75% and 100% mineral fertilizer, with and without biostimulant) showed significantly higher total dry matter yield (p = 0.0016–0.0337; Table 3).
To evaluate differences between reduced fertilization treatments with biostimulants (F75_BIO3, F75_BIO6, F75_BIO12) and full mineral fertilization (F100_BIO0), Tukey pairwise comparisons were performed (Table A2). These showed no statistically significant differences between treatments (p > 0.9).
These results suggest that the primary driver of increased dry matter yield in this experimental design was mineral fertilizer supply, while the contribution of the biostimulant may be interpreted as a modulation of input efficiency rather than evidence of replacement of mineral fertilizers.

3.3. Multivariate Analysis of Substrate and Biostimulant Effects

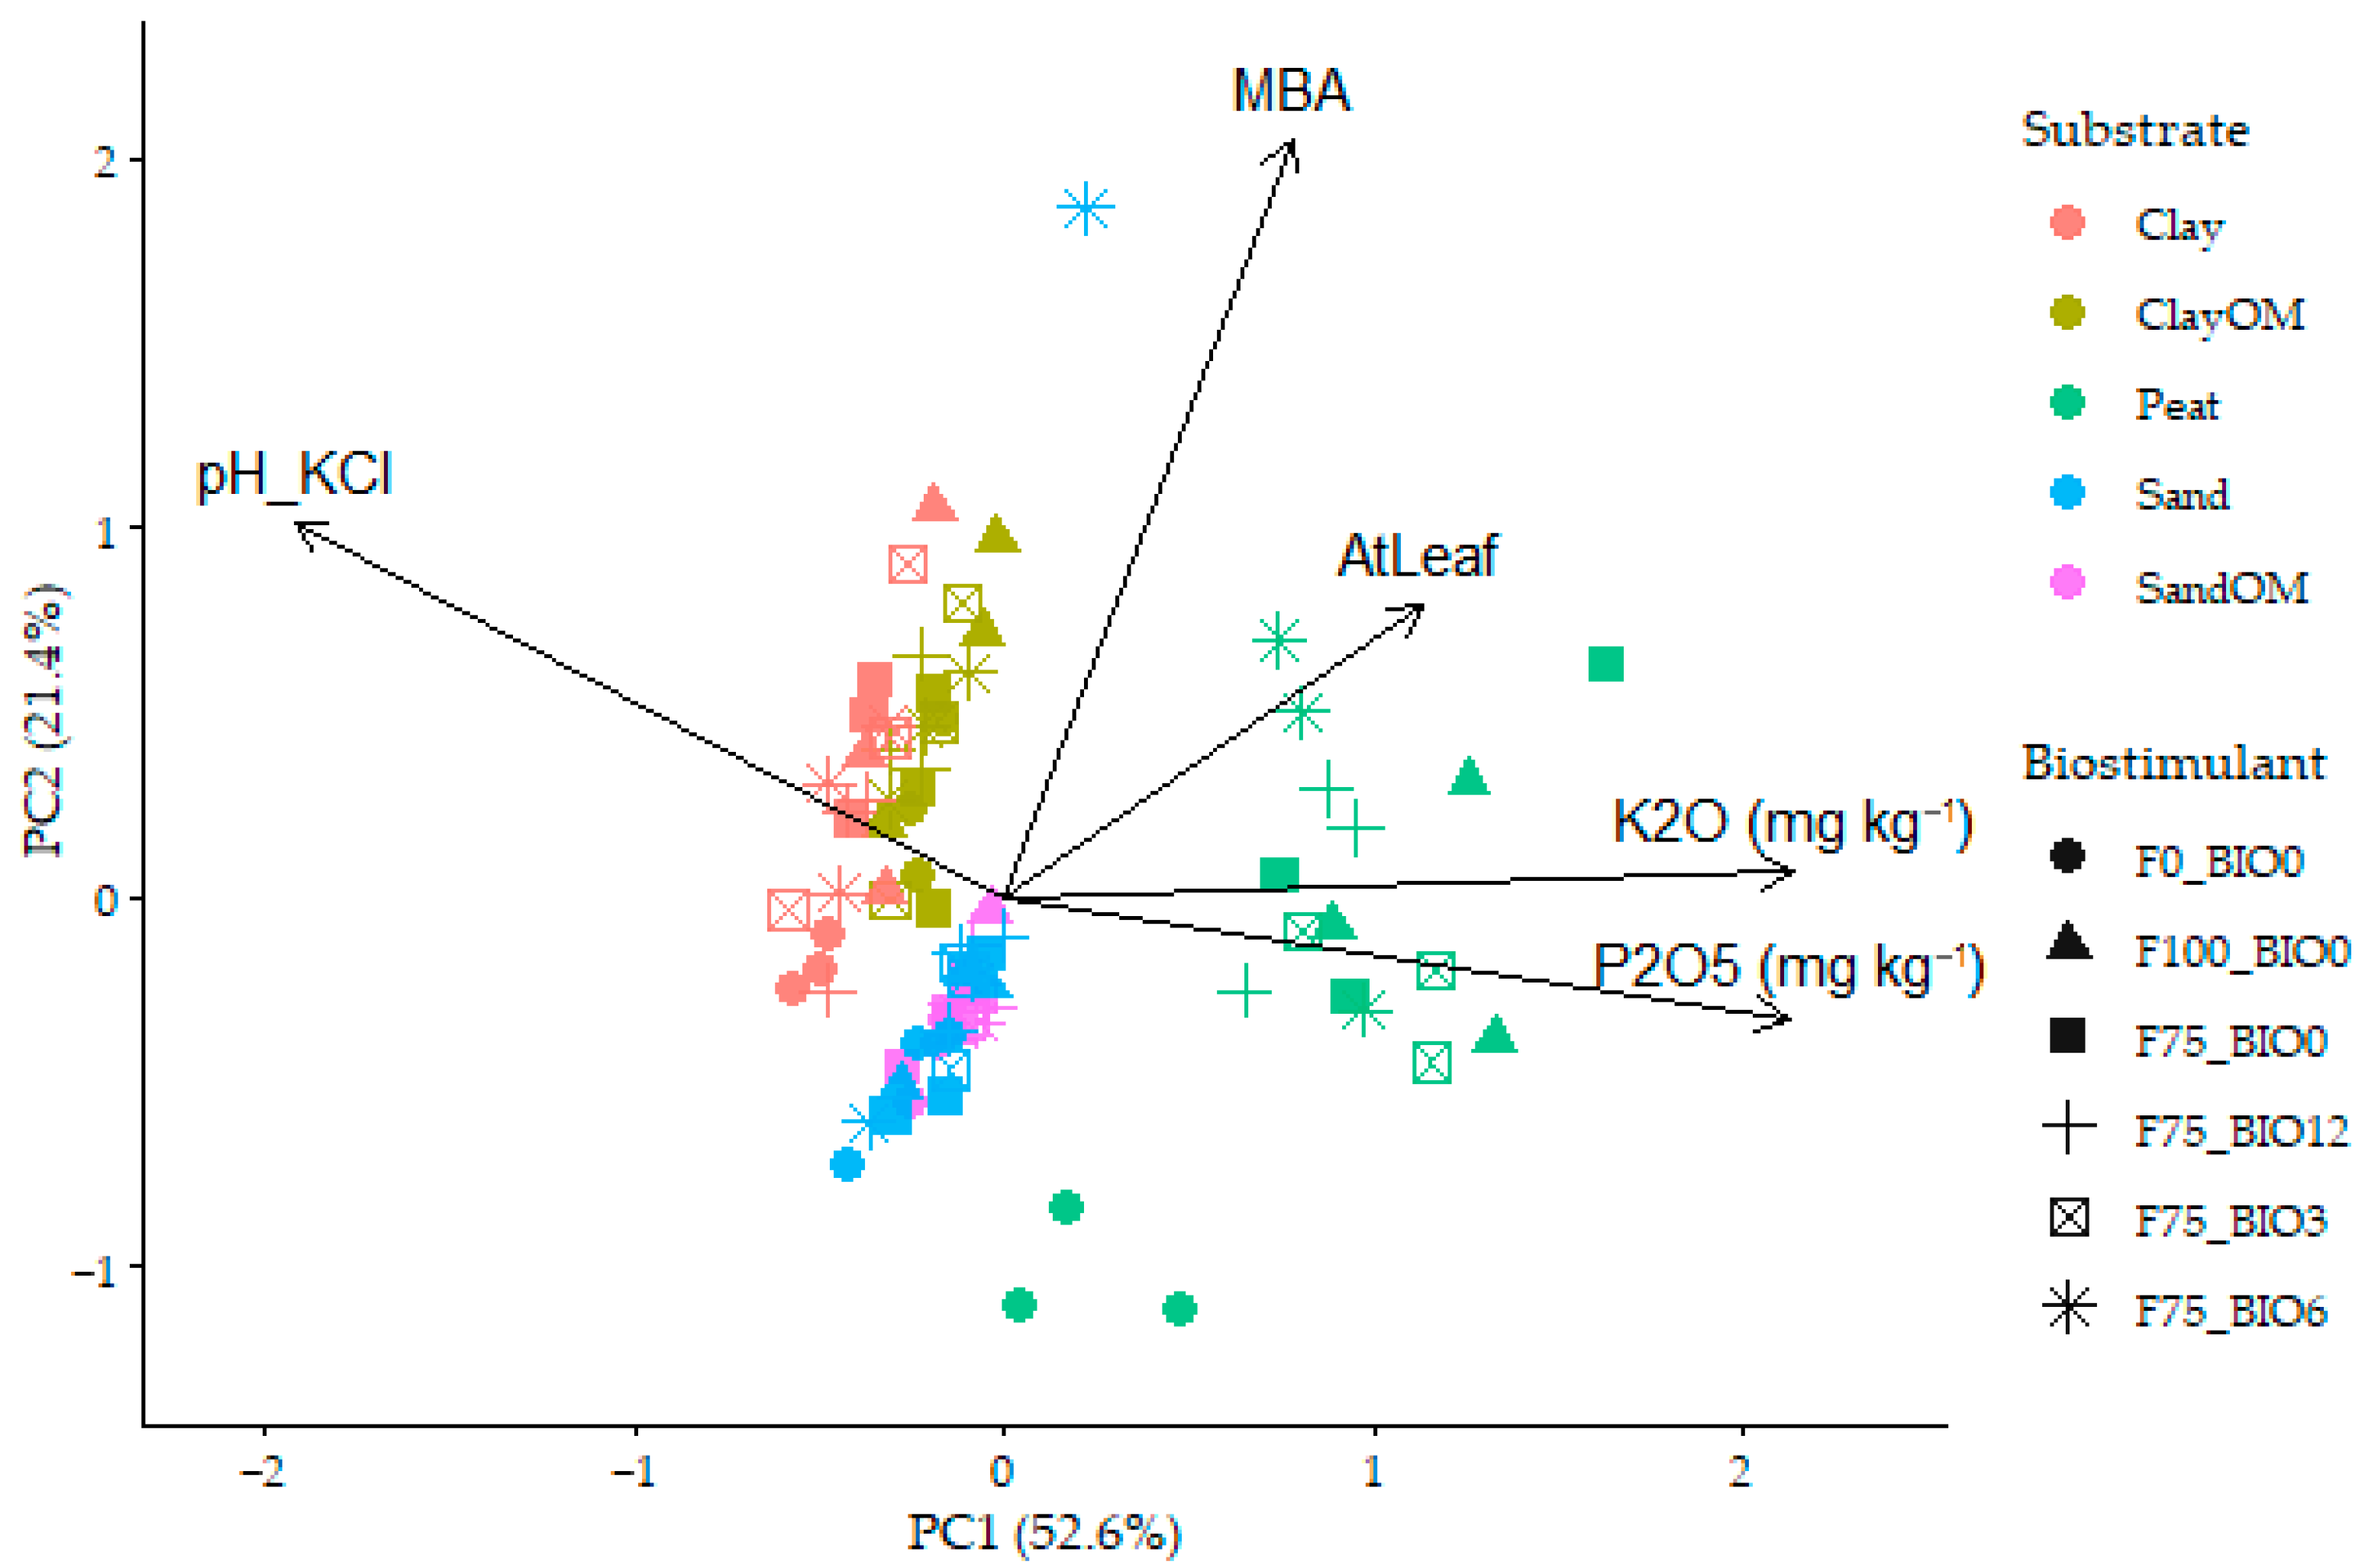
Principal component analysis (PCA), incorporating soil chemical, microbial, and plant development indicators, revealed a clear spatial separation of substrates in the ordination space. The first principal component (PC1) explained 52.6% of total variation and was closely associated with post-harvest P2O5 and K2O content in the substrate, thus reflecting the chemical background of substrates following cultivation. The second principal component (PC2), which explained 21.4% of the variation, was associated with soil microbial activity (MBA) and the rate of leaf development (Figure 3) MBA contributed to the separation of samples along PC2, although no consistent statistically significant differences between treatment variants were observed.
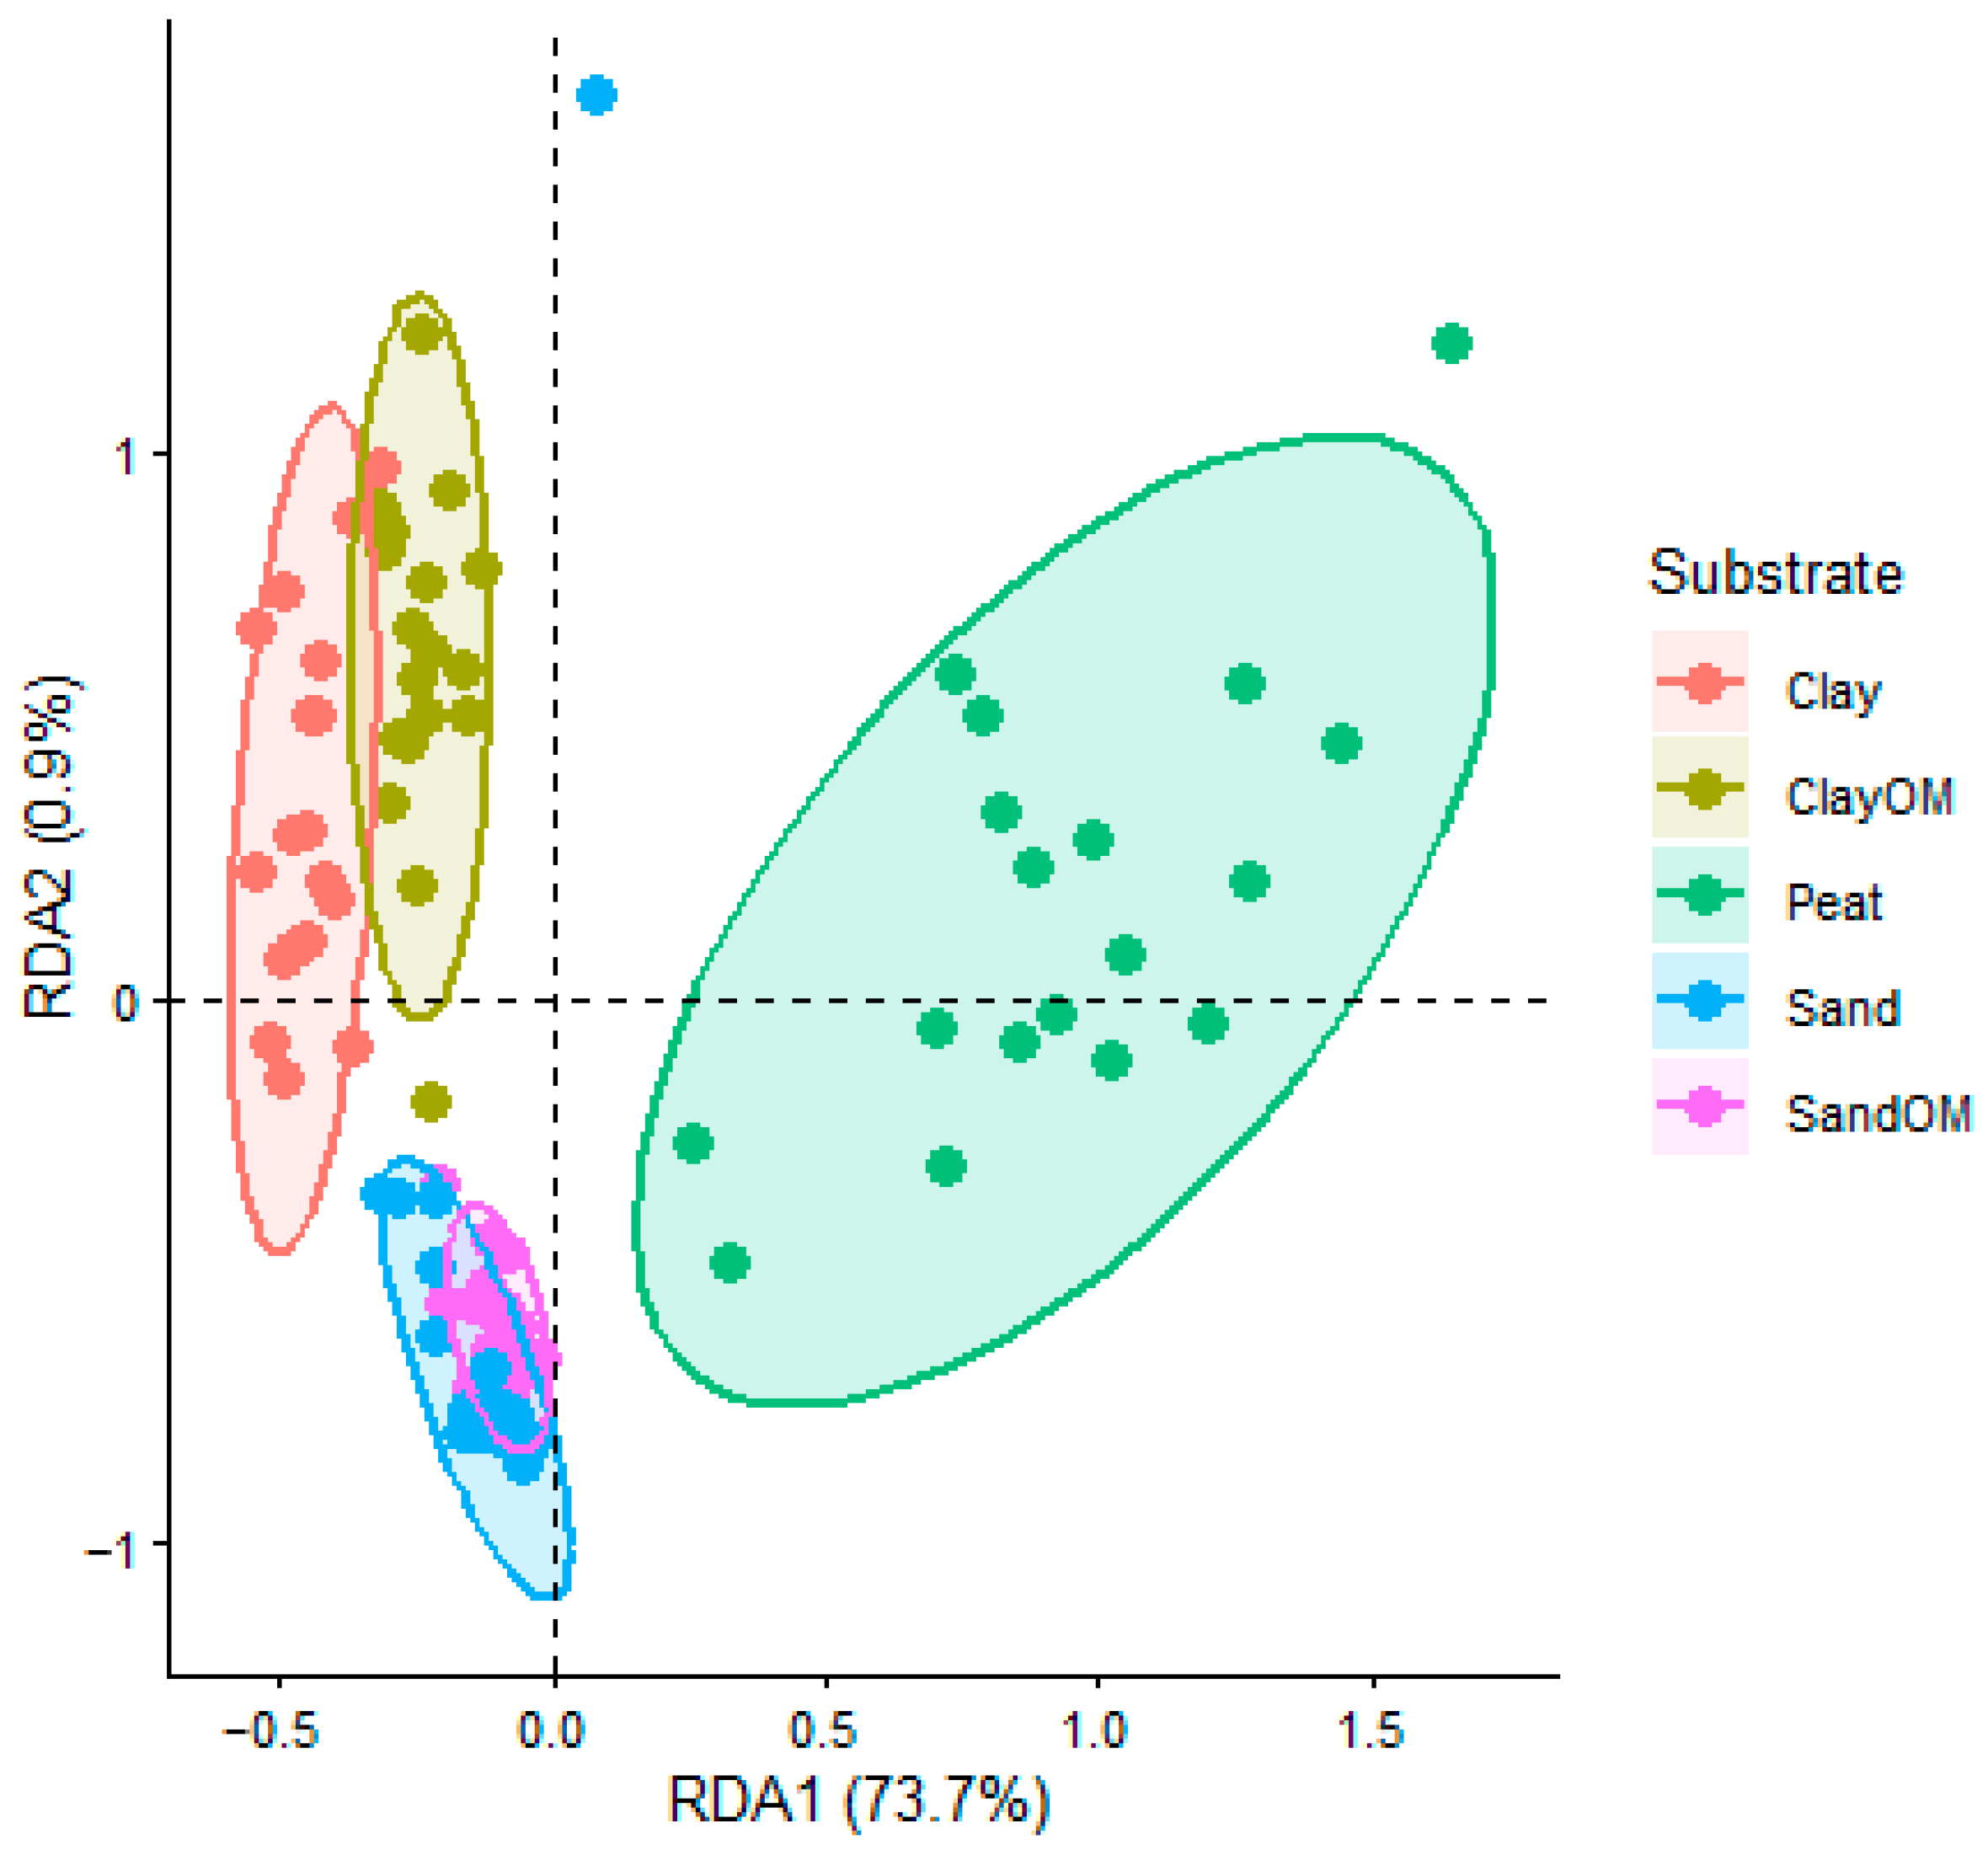
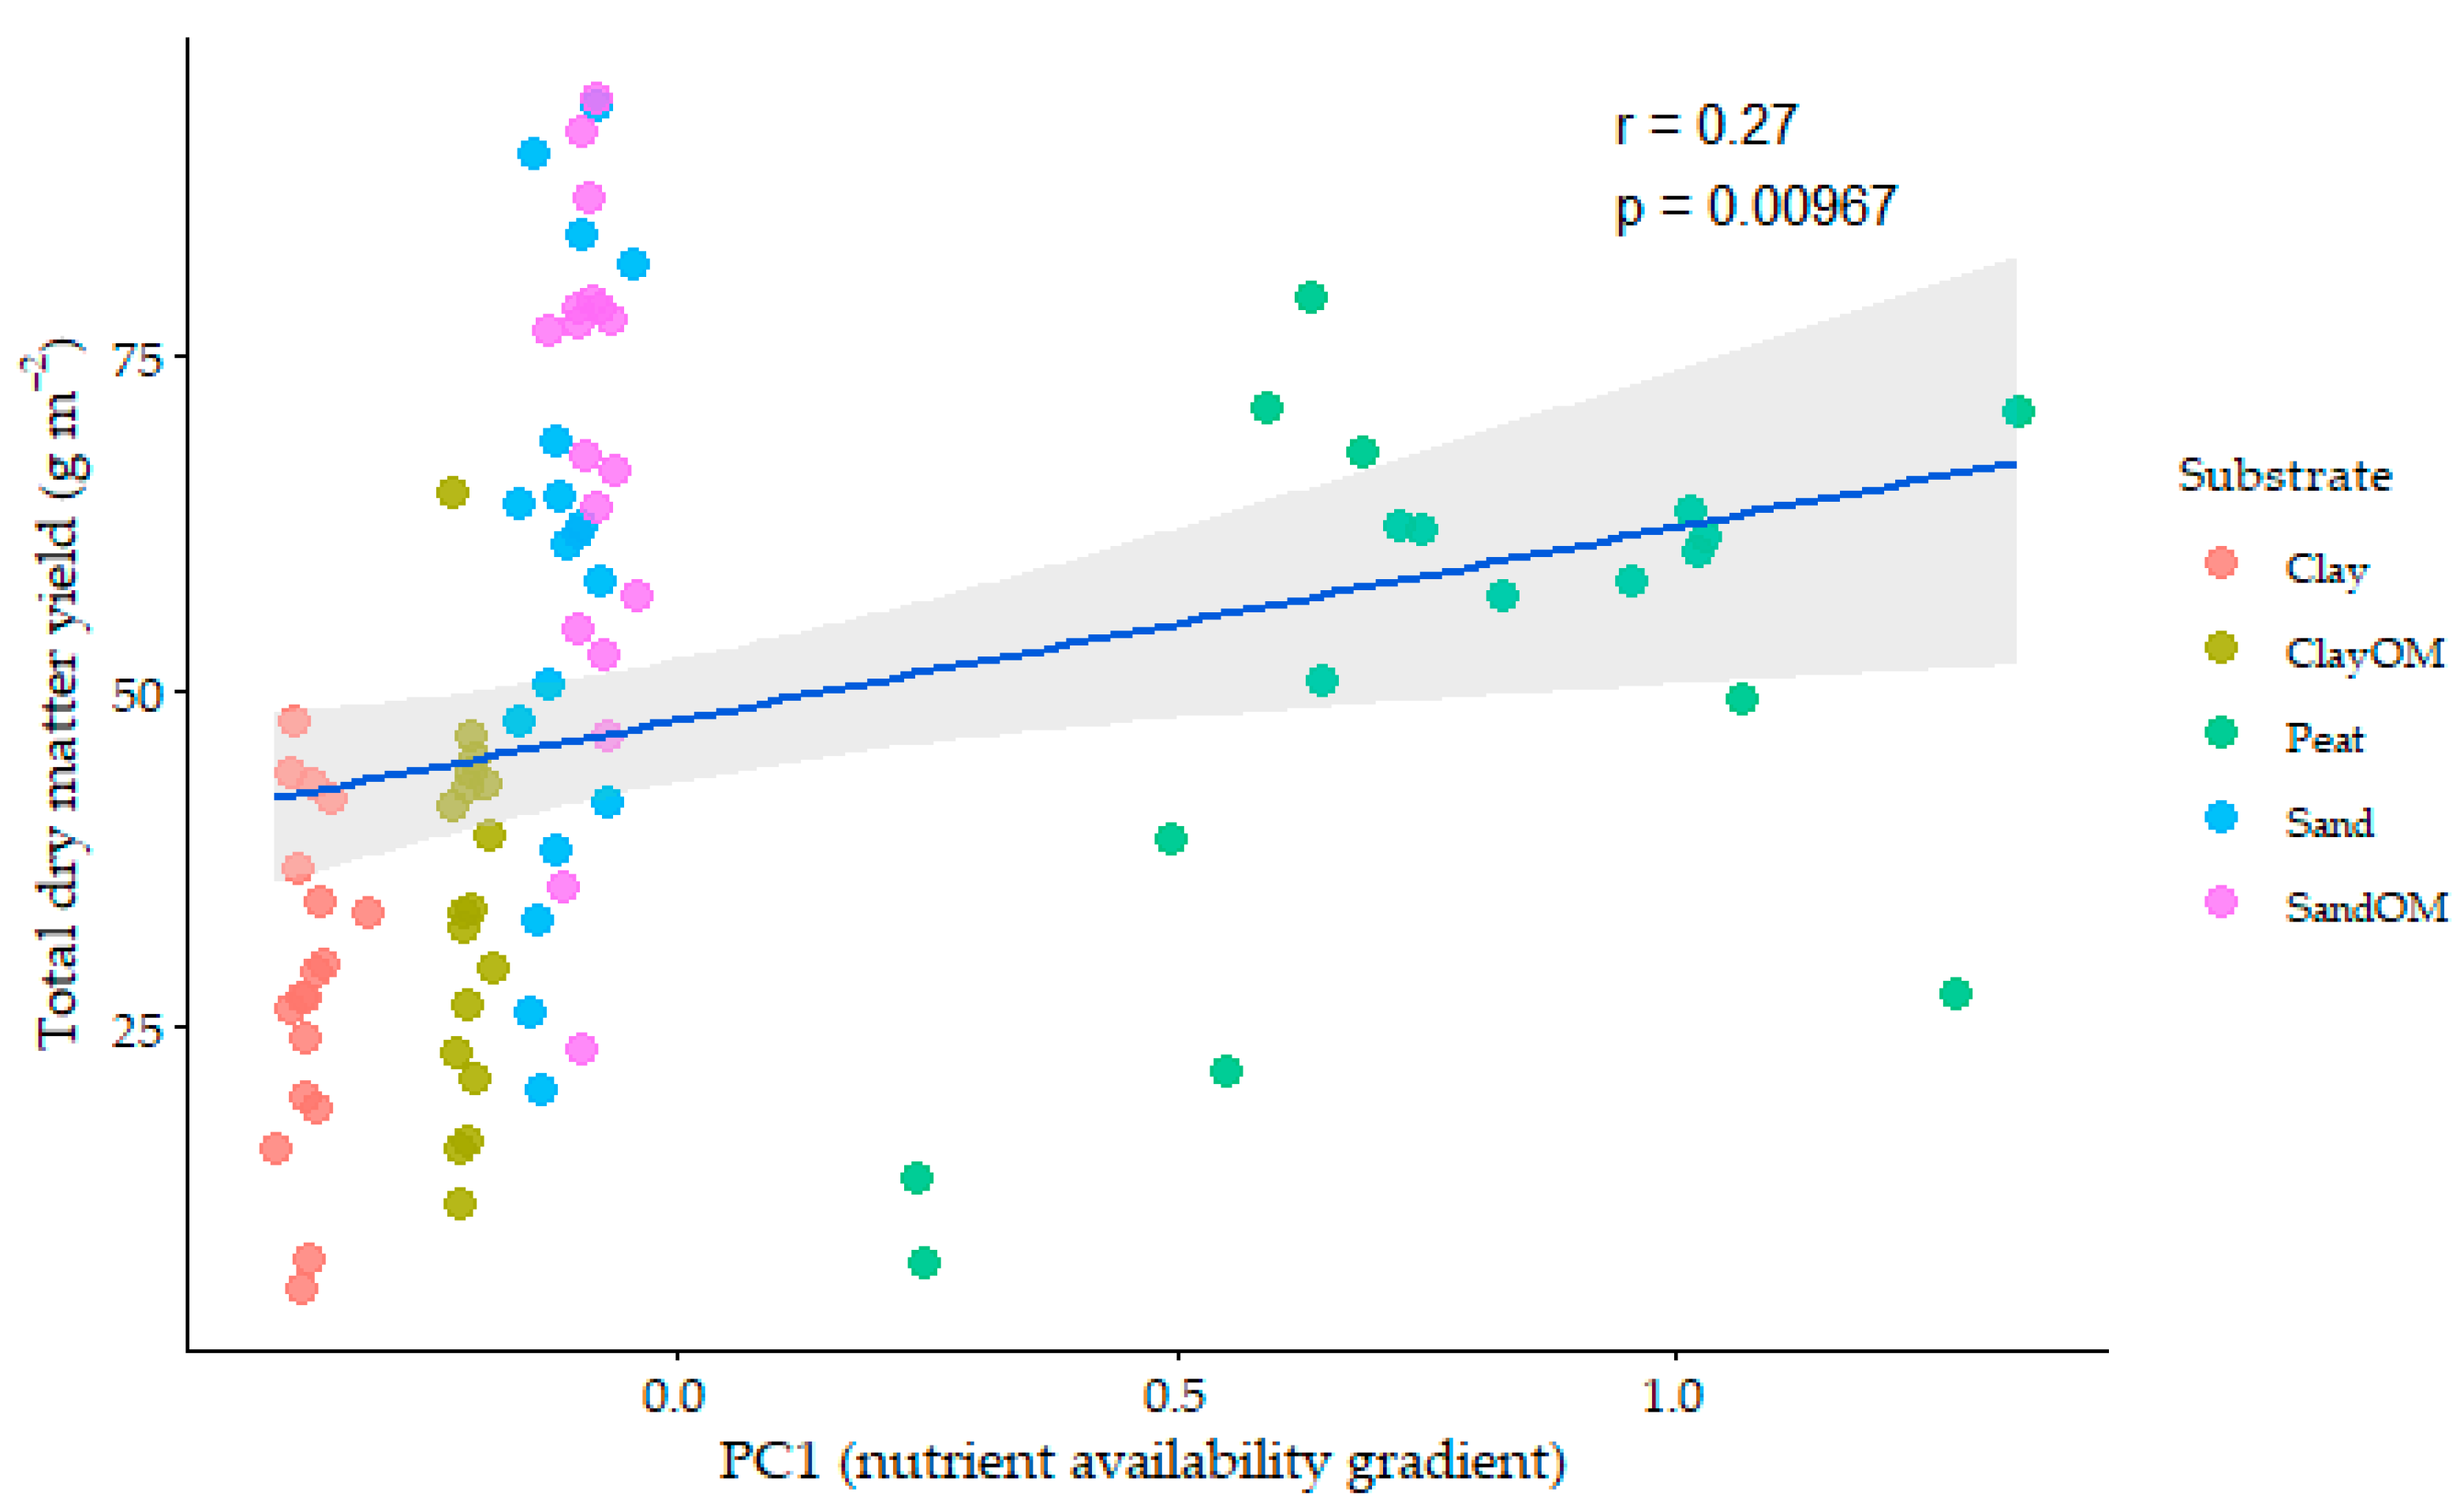
Total dry matter yield showed a weak but statistically significant positive association with PC1 (r = 0.27, p = 0.0097), thus indicating that yield tended to increase along the primary chemical gradient identified by the PCA (Figure A2, Appendix A). The permutation test in the redundancy analysis (RDA) revealed that substrate type had a significant effect on the multivariate structure of soil and plant variables (p = 0.001), while the contribution of the treatment factor was also statistically significant but markedly smaller (p = 0.024) and did not translate into substantial changes in total dry matter yield (Table A1, Appendix A).
The RDA ordination was primarily structured along the RDA1 axis, which explained 73.7% of the canonical variation and reflected a marked separation of the peat substrate relative to mineral substrates, which formed more closely grouped clusters. The effect of treatment variant in the ordination space was less pronounced and consisted primarily of subtle variation in sample distribution within substrates (Figure 4).
Substrate-level correlation analysis showed that total dry matter yield was positively associated with leaf development rate (AtLeaf) and soil potassium content (K2O), with correlation in the range r = 0.51–0.61 (p < 0.05).
Analysis of the leaf development indicator (AtLeaf), using a linear model with total dry matter yield, substrate type, and biostimulant variant as explanatory variables, showed that biostimulant variant had a significant effect on AtLeaf (F (5.79) = 2.86, p = 0.0043). The substrate effect was not statistically significant (p > 0.12). Compared with the unfertilized control (F0_BIO0), all biostimulant variants showed statistically significant increases in AtLeaf (Δ = 5.34 to 7.58; p = 0.004–0.036), but no statistically significant differences were observed between biostimulant variants (Tukey HSD, p > 0.08). The total dry matter yield was not a statistically significant determinant of AtLeaf (β = 1.59 ± 1.48; p = 0.285).

3.4. Illustrative Cost Scenario for Reduced Mineral Fertilization

Based on mineral fertilizer doses used in the experiment and typical radish fertilization rates in the Baltic region, this section presents a conceptual economic analysis based on literature-derived cost data. The full mineral fertilizer dose (100% NPK) was estimated to cost EUR 162–242 ha−1, while reducing the dose to 75% resulted in costs of EUR 121–182 ha−1. The estimated cost difference between the two scenarios was EUR 40–61 ha−1 (Table 4). It should be noted that the economic outcome is sensitive to yield variability, and even small changes in yield may substantially influence the overall economic balance.
The cost calculations use typical radish fertilization standards in the Baltic region (100–150 kg N ha−1, 80–120 kg P2O5 ha−1, 120–180 kg K2O ha−1) and mineral fertilizer prices projected for 2025 [19,20,21,22,28,29,30,48,50]. The cost of the full 100% NPK dose was estimated at EUR 162–242 ha−1 using the formula (N dose × 0.60) + (P2O5 dose × 0.55) + (K2O dose × 0.48). The 75% scenario reduces costs proportionally to EUR 121–182 ha−1, yielding estimated savings of EUR 40–61 ha−1.
In addition to the comparison of mineral fertilizer costs, this study conceptually evaluated the costs of obtaining and applying Furcellaria lumbricalis digestate, based on literature-derived estimates rather than direct measurement. Based on anaerobic fermentation studies of seaweed biorefineries and coastal algae, the farm-level cost of digestate was estimated at EUR 20–30 ha−1, encompassing biomass collection, fermentation, digestate storage, transport, and application [19,20,21,22,28,29,30,50]. This interval does not reflect the 30 L laboratory-scale reactor used in this study but reflects literature-derived cost levels for small- to medium-scale pilot projects in the Baltic Sea region [19,20,21,22,28,29,30].
Combining the estimated fertilizer savings associated with a 25% reduction in mineral fertilizer input (EUR 40–61 ha−1) with literature-based digestate cost estimates (EUR 20–30 ha−1) suggests a potential cost balance of EUR 10–41 ha−1 in favor of the 75% NPK + digestate scenario. This estimate is illustrative only, does not reflect the actual laboratory-scale production costs of this study, and should be interpreted as a conceptual scenario requiring validation under pilot and commercial conditions.

4. Discussion

4.1. Equivalence of Yield at Reduced Mineral Fertilizer with Biostimulant

This study found that, in certain substrates, 75% mineral fertilizer combined with Furcellaria lumbricalis digestate maintained dry matter yields that were not statistically different from 100% mineral fertilizer alone (Figure 2). These results suggest similar yield levels; however, no statistically significant differences between F75_BIO and F100_BIO0 were observed (Tukey’s HSD, see Appendix A, Table A2). Although no statistically significant differences were found between biostimulant dose options (3%, 6%, and 12%), estimated marginal means showed that the highest dose (12%) in clay and clay-with-organic-matter substrates reached levels comparable to full mineral fertilizer. These results are consistent with previously published observations on the biostimulating properties of seaweed extracts, in which improved NUE and plant productivity at reduced mineral fertilizer input were demonstrated [7,14,51].
Meta-analyses of the effects of seaweed biostimulants on yields report average yield increases of 15–17% across different crops, with more pronounced effects for extracts of red algae (Kappaphycus alvarezii, Gracilaria spp.): maize (+18.54%), tomatoes (+12–25%), and soybean (up to +30% under stress) [14,15,16,52]. These meta-analytical trends suggest that seaweed digestates may function not only as supplementary nutrient sources, but also as carriers of bioactive compounds that modulate plant metabolism and stress tolerance [7,13]. The similarity in mean yields observed at 75% NPK with biostimulant addition is consistent with this body of literature: the biostimulant does not produce a substantial yield increase above full mineral fertilizer but may contribute to maintaining agronomic productivity under reduced NPK input, although this was not statistically confirmed.
The effect of the biostimulant was context-specific: no statistically significant effect on total dry matter yield was detected, although modeled values and confidence intervals indicated positive trends in certain substrate types. This finding is consistent with other studies documenting variable efficacy of seaweed biostimulants depending on soil type, organic matter content, and pH [10,25]. Li et al. (2022) [53] demonstrated that the effect of the liquid fraction of digestate on vegetable crops varied significantly between mineral and organic substrates, with stronger effects in peat and composted substrate variants. Correspondingly, the biostimulant effect in this study was more pronounced in clay substrates and sand with organic matter, while a negative trend was observed in the pure sand substrate.
At the physiological and biochemical level, the positive effects of seaweed biostimulants, especially from red algae (Rhodophyta), on NUE can be attributed to several parallel mechanisms [7,13,27].
  • Biochemical and physiological modulation: the presence of carrageenans and other bioactive compounds may stimulate root system development by enhancing nutrient uptake capacity [17,18].
  • Enhanced photosynthetic efficiency: seaweed extracts significantly increase chlorophyll a and b content (+20–107% in various studies) through improved Mg2+ uptake and upregulation of Photosystem II protein expression [54,55].
  • Rhizosphere microbiome modification: Kappaphycus-based biostimulants enrich rhizosphere populations of Proteobacteria and Actinobacteria, which are associated with microbial processes related to nitrogen cycling and phosphorus mobilization.
  • Metabolic reprogramming: transcriptomic analyses show that seaweed biostimulants upregulate genes involved in primary metabolism (carbon fixation and nitrogen assimilation) and stress response pathways (HSP, dehydrins) [13,16].
These mechanisms may help explain why biostimulants can sustain yields at a reduced NPK dose: not by replacing nutrients, but by improving nutrient use efficiency and plant physiological status. The results of this study, in which 75% NPK combined with biostimulant meant that yields were similar to those of the full NPK dose, are consistent with the NUE improvement framework described in the literature [6,7,8], although no statistically significant differences were detected.
The economic dimension is relevant in the context of fertilizer price volatility resulting from the Russia–Ukraine conflict (+43% increase in nitrogen fertilizer prices and +28% for phosphorus in 2022–2024): a 25% reduction in NPK dose yields cost savings of EUR 40–61 ha−1 for radishes (Table 4) based on literature-derived estimates [1,3,5]. Such a partial replacement strategy may be economically justified if the cost of producing and applying the biostimulant is lower than the value of the mineral fertilizer saved. These estimates require further validation under field conditions with different crops and economic models.
The results indicate that Furcellaria lumbricalis digestate from the Baltic Sea may help maintain radish dry matter yield at 75% of the NPK dose in certain substrates, with mean values approaching those observed under full mineral fertilizer. Although biostimulant effects on absolute yield were not always statistically significant, positive effects on plant physiological parameters (AtLeaf index and microbial activity) were observed, supporting the potential of biostimulants as tools for nutrient recycling and NUE improvement in the circular bioeconomy context [38,44,45]. Further studies are needed to: (1) validate these effects under field conditions for different crops; (2) optimize the dose and timing of biostimulant application according to substrate type; (3) quantify effects on product quality and storability; and (4) conduct full life-cycle analyses (LCA) comparing environmental impacts with those of synthetic fertilizers [34,35,36].
Overall, the results do not provide statistical support for the hypothesis that Furcellaria lumbricalis digestate can substitute for mineral fertilizer while maintaining yield under the conditions of this study, although some trends were observed across substrates.

4.2. AtLeaf Index and Photosynthetic Efficiency

Studies on Kappaphycus alvarezii in recent years have reported that marine algae biostimulants exert positive effects on different crops under certain conditions, contributing to surface biomass growth, root development, and nutrient efficiency, increasing chlorophyll content and photosynthesis rates, and influencing the rhizosphere microbiome [11,15,16]. Studies of the AgroGain® biostimulant with cucumber and maize have shown that products derived from Kappaphycus alvarezii simultaneously stimulate shoot and leaf growth, increased chlorophyll, carotenoid, and soluble carbohydrate contents, reduce plant stress responses, and modify the rhizosphere microbial community [11,16]. Similarly, studies with Gracilaria extracts report a +20–107% increase in chlorophyll content [7,54,55], attributed to: (i) improved Mg2+ uptake required for chlorophyll biosynthesis; (ii) increased expression of Photosystem II reaction center proteins; and (iii) optimized chloroplast ultrastructure and thylakoid membrane organization [7,13]. However, it should be noted that the effects of biostimulants are strongly influenced by raw material origin and processing technology, and therefore may differ between seaweed extracts and anaerobically derived digestates. The increase in AtLeaf index observed in all biostimulant variants in this study (Δ = +5.34 to +7.58; p = 0.004–0.036), together with similar dry matter yield at 75% mineral fertilizer in some substrates, is broadly consistent with trends reported in previous studies, despite the use of a different species (Furcellaria lumbricalis) and a different technological process (digestate rather than extract). These results suggest that locally available Baltic Sea resources can exhibit biostimulating properties consistent with those of seaweed products described in the literature, while reducing dependence on imported raw materials [11,12,13]. These findings complement current research on next generation biostimulants, highlighting the potential of native seaweed-derived products as functionally and biologically active solutions [8,10,56].
Recent research on next generation biostimulants reflects a transition from traditional, empirically characterized extracts to more precisely defined molecular and microbial activity profiles, including seaweed derivatives, pure bioactive compounds, and nanomaterials [8,10,56].

4.3. Microbial Activity and Substrate–Biostimulant Interaction

As discussed in the Introduction, seaweed-derived biostimulants may influence soil biological processes through interactions with the microbial community. In the present study, this aspect was indirectly addressed through the assessment of microbial biomass activity (MBA) as an indicator of overall soil biological activity. The linear mixed model results indicate that substrate type and treatment variant affected total dry matter yield, but their interaction was not statistically significant. This indicates that the relative impact of treatment variants was generally consistent across substrates, although more pronounced descriptive trends were observed in certain cases. Studies with digestates and biostimulants have reported that statistically non-significant but consistent trends may reflect biological processes that require larger, more targeted datasets for full characterization [24,25]. Higher biostimulant doses in the clay substrate tended to be associated with higher mean dry matter yield values approaching levels observed under full mineral fertilizer treatment, while individual doses in sand with organic matter showed similar or slightly higher mean values than the full mineral fertilizer variant. These observations are descriptive and based on a limited dataset; they indicate a possible substrate-specific response to biostimulant doses and justify more comprehensive targeted studies. Previous studies with digestates from anaerobic fermentation have demonstrated yield equivalence with mineral fertilizers under certain conditions, with outcomes depending on soil type, cultivation system, and management intensity [24,25]. The results obtained are consistent with biostimulant modulation rather than a transformative mechanism of action, whereby it affects existing biological processes without fundamentally altering substrate properties [6,7,8,10]. However, microbial community composition and specific functional processes were not directly assessed in the present study.
The effects reported in the literature of seaweed biostimulants on the soil microbiome indicate that carrageenans and other polysaccharides can serve as selective substrates for beneficial bacteria (Proteobacteria and Actinobacteria), potentially supporting microbial processes related to nitrogen cycling and phosphorus mobilization [13,16,18]. Such rhizosphere microbiome modifications may produce synergistic effects beyond direct nutrient additions and explain yield maintenance at reduced NPK levels [10,16]. These mechanisms are discussed here as literature-based explanatory context only; they were not directly measured in the present study and therefore should not be interpreted as directly demonstrated mechanisms of action for Furcellaria lumbricalis digestate in this experiment.

4.4. Impact of Substrate Properties and LCA Perspective

It should be noted that in this study, Furcellaria lumbricalis digestate was produced using a 30 L laboratory-scale anaerobic fermentation reactor (RTU, Liepaja, Latvia) optimized for process control and data logging rather than for cost minimization or scale-up. Consequently, the technological solution applied here is not directly representative of commercial cost levels, and all economic conclusions should be interpreted as conceptual, based on cost intervals reported in the literature for marine algae biorefinery and digestate application systems [21,22,28,29,30].
Life cycle assessment (LCA) of the Furcellaria lumbricalis biostimulant production process indicates that the most significant environmental and cost hotspots are reactor heating and digestate stream management, with optimization potential through process scale-up to pilot in commercial facilities and integration of renewable energy [34,35,36,38,39,44]. Published LCA results for marine algae biorefineries demonstrate that anaerobic fermentation with biogas and digestate co-production can achieve a positive environmental balance when biogas replaces fossil fuels and digestate replaces synthetic fertilizers [34,35,36,37]. Seghetta et al. (2016, 2017) demonstrated that marine algae biorefineries in northern Europe can reduce greenhouse gas emissions by 30–50% compared to conventional systems when energy recovery and nutrient recycling are optimized [35,36]. The 25% mineral fertilizer reduction scenario proposed in this study may therefore be considered to be an agronomically founded and economically viable approach whose full evaluation requires integrated analysis at the farm level and across the life cycle [34,35,36,38,39,44]. However, given that the effects on yield were not always statistically significant, these conclusions should be interpreted with caution and primarily reflect indicative trends rather than definitive outcomes.
Differences in post-harvest P2O5 and K2O residues between peat and mineral substrates reflect markedly different substrate chemical backgrounds and buffer capacities rather than direct nutrient availability to plants during growth. The PCA and RDA results indicate that substrate type was the dominant factor structuring the multidimensional variation in the soil–plant system, while the biostimulant treatment accounted for a smaller but statistically significant proportion of variance [57,58,59]. PC1 explained 52.6% of total variation and was closely associated with post-harvest P2O5 and K2O content and total dry matter yield, representing a nutrient fertility gradient from low-nutrient mineral substrates (negative PC1 values) to nutrient-rich organic substrates (positive PC1 values). PC2 explained 21.4% of the variation and was associated with soil microbial activity and plant physiological parameters. Redundancy analysis quantified the relative contributions of the canonical variation and reflected primarily the effect of substrate type (F = 55.55; p = 0.001), confirming substrate type as the primary factor structuring response variability. The biostimulant variant contributed a smaller but statistically significant proportion of variance (F = 2.53; p = 0.024), consistent with a modulating rather than transformative mechanism of action [24,25,57,58]. These results emphasize that interpretation of biostimulant effects without the context of substrate type and organic matter content may be incomplete. The interaction between these factors with biostimulant dose may determine both the direction and magnitude of the response—a finding that may explain the conflicting results reported in the biostimulant efficacy literature [10,25,59].

4.5. AtLeaf Indicator and Crop Correlation

The AtLeaf index was significantly higher in all biostimulant variants compared to the unfertilized control (F0_BIO0), but did not show consistent differences among the 3%, 6%, and 12% doses; no statistically significant association was found with total dry matter yield (r = 0.10; p = 0.285). These interpretations are supported by existing literature and provide a possible explanation of the observed patterns. The weak correlation between the AtLeaf index and total dry matter biomass may be explained by several factors.
  • Point measurement vs. cumulative biomass: AtLeaf measurements record chlorophyll concentration at the individual leaf level, while total plant biomass accumulation depends on the integrated interaction of leaf area, chlorophyll concentration, and light interception efficiency [7,54,55].
  • Source–sink balance: improved chlorophyll content increases photosynthetic source capacity, while biomass storage requires adequate sink strength (root growth and storage organ development) to utilize photosynthate [10,17,18].
  • Temporal offset: AtLeaf measurements were recorded at specific time points, whereas total dry matter mass represents cumulative biomass across all growth periods. Biostimulant-induced increases in chlorophyll occur predominantly in early growth stages but may diminish before harvest, resulting in weak correlation with final yield [15,16,55].
This pattern is consistent with recent studies in which chlorophyll indices and photo-physiological parameters respond more rapidly and sensitively than yield indices; biostimulant effects on physiology are often expressed across a wider dose range, while the yield response curve is more linear or substrate dependent [11,13,15,16]. In this context, AtLeaf serves as an early indicator of nutritional and stress status reflecting biostimulant exposure, but is not the sole criterion for dose optimization.

4.6. Circular Bioeconomy and the Potential of the Baltic Region

To place the experimental findings in a broader agronomic and sustainability context, a conceptual assessment of the circular bioeconomy potential of Furcellaria lumbricalis was performed. This analysis builds on the observed tendency of the digestate to maintain yield at reduced (75%) mineral fertilizer rates in certain substrates and explores potential implications for resource efficiency and nutrient recycling. The biomass of Furcellaria lumbricalis can be collected from material washed ashore after autumn storms in the Baltic Sea without damaging underwater algal populations, as reported in the literature [38,44,45]. This form of biomass collection is generally considered to have low environmental impact because the biomass would otherwise go unused [37,44]. Previous studies have described Furcellaria lumbricalis biomass valorization as a multi-flow system in which several interlinked value streams can be derived from coastal biomass [37,38,44,45].
  • Coastal biomass collection as an environmental management service (approximately EUR 10–20 tonne−1 environmental service value) [37,44].
  • Renewable energy: biogas (55–65% CH4, approximately 4–6 MWh tonne−1 dry matter biomass, approximately EUR 600–900 tonne−1 energy revenue at EUR 150 MWh−1) [28,29,30].
  • Agronomic biostimulant production (approximately EUR 20–30 tonne−1 market price potential) [44,45].
  • Climate change mitigation: a 25% reduction in NPK prevents Haber–Bosch emissions (approximately 2 kg CO2-eq kg−1 N) and reduces phosphate mining impacts [1,3,5,34,35,36].
These integrated systems align with EU Bioeconomy Strategy priorities [31,32,33,37]. Beyond the direct production economy, Furcellaria lumbricalis digestate production may support rural employment (harvesting, processing, and distribution), reduces foreign currency outflows for mineral fertilizer imports (approximately 90% import dependence in Latvia, Estonia, and Lithuania), and improves supply chain resilience [38,44,45]. Based on volumes reported in the literature, the accumulation of Furcellaria lumbricalis beach-cast material in Latvia and Estonia is estimated at approximately 5000–15,000 tonnes dry matter per year, potentially sufficient to produce approximately 500–1500 tonnes of liquid digestate. These estimates are based on literature-derived data and should be interpreted as indicative of potential rather than precise production capacity. At a 6% (v/v) application rate of 10 L m−2, this quantity could supply approximately 1000–3000 hectares of horticultural production [37,44,45].
Life cycle analyses of marine algae biorefineries in northern Europe demonstrate that integrated systems with biogas and digestate co-production may achieve 30–50% reductions in CO2-eq emissions compared to fossil fuel alternatives when energy recovery and nutrient recycling are optimized [34,35,36,37]. Alvarado-Morales et al. (2013) and Seghetta et al. (2016, 2017) identify the most significant environmental hotspots as transport distances (>50 km negatively affecting the balance) and reactor energy consumption (heating, milling) [34,35,36]. The compact coastal infrastructure and short transport distances characteristic of the Baltic region (<30 km from beach to fermentation facility) may contribute to a favorable LCA balance [37,38,44]. However, a full LCA comparing the 75% NPK + digestate and 100% NPK scenarios is required to quantify eutrophication, acidification, and resource depletion impacts [34,35,36,37].

4.7. Practical Implications and Future Research Directions

The results of this study indicate that locally available Furcellaria lumbricalis digestate from the Baltic Sea may support maintaining total dry matter yield of garden radish in certain substrates when mineral fertilizer input is reduced to 75% of the full norm, offering a practical approach to optimizing mineral fertilizer consumption in the context of resource price volatility. Positive effects of the biostimulant on leaf development indicators (AtLeaf) and substrate–plant system functioning, as revealed by multivariate analyses (PCA and RDA), suggest that the role of digestate lies primarily in modulating input efficiency and stabilizing physiological processes rather than fully replacing mineral fertilizers [19,20,21,22,23,34,35,36,37]. In practical terms, Furcellaria lumbricalis digestate may serve as an option for partial reduction of mineral fertilizer inputs in intensive vegetable production, particularly on substrates with sufficient organic content and buffer capacity, where estimated cost savings (EUR 40–61 ha−1 in the 75% NPK scenario, based on literature-derived estimates) can be combined with potential benefits from improved nutrient efficiency. Substrate-level analysis shows that digestate efficacy is strongly dependent on the physicochemical properties of the substrate, and that biostimulant addition to organic-free sandy substrates does not yield the same results as in substrates with higher organic content, a finding that should inform regionally adapted recommendations.
The observed substrate-dependent response patterns reflect the complexity of the substrate–plant–biostimulant system and suggest that larger and more targeted datasets would further improve the resolution of biostimulant effects across different growing conditions.
In the policy and bioeconomy context, the use of Furcellaria lumbricalis digestate in integrated biorefineries may offer opportunities to address coastal biomass management, renewable energy production and nutrient recycling challenges simultaneously, thus supporting implementation of circular bioeconomy models in the Baltic Sea region [31,32,33,34,35,36,37,38,39]. Empirical data on locally sourced digestate across diverse substrate types provide the basis for practical recommendations and serve as input for further life cycle and economic analysis, including scenarios with higher fertilizer price levels and evaluation of additional crops [34,35,36,37,38,39,44,45].
Future studies should extend testing of Furcellaria lumbricalis digestate beyond pot experiments to field trials under diverse agro-ecological conditions, validate the results and assess biostimulant effects on yield stability across multiple growing seasons [19,20,21,22,23,28,29,30]. Integration of molecular and microbial parameters, including rhizosphere microbiome structure and plant gene expression profiles, with multi-factor statistical analyses is essential for further understanding of substrate–biostimulant interaction mechanisms and for developing targeted recommendations for sustainable agriculture applications [11,12,13,57,58,59].

5. Conclusions

  • The impact of Furcellaria lumbricalis digestate on total dry matter yield depended on substrate type at a 75% mineral fertilizer rate. In certain substrates, biostimulant application was associated with higher modeled dry matter yields values; however, in most cases, differences between digestate doses were not statistically significant.
  • A two-factor linear mixed-model analysis revealed that substrate type and treatment variant significantly affected dry matter yield. Their interaction was not statistically significant, indicating a generally consistent pattern of treatment effects across substrate types.
  • Multivariate analysis (PCA and RDA) showed that substrate type was the dominant factor in the structure of soil and plant parameters, while biostimulant variants contributed a statistically significant but relatively small proportion of variance, which did not translate into significant changes in total dry matter yield.
  • Biostimulant application was associated with a statistically significant increase in leaf development rate (AtLeaf) compared to the unfertilized control, but no significant differences were found among biostimulant doses and AtLeaf was not directly related to total dry matter yield.
  • A conceptual cost scenario based on literature-derived estimates suggests that reducing mineral fertilization to 75% and supplementing it with Furcellaria lumbricalis digestate may lower mineral fertilizer expenditure by approximately EUR 40–61 ha−1. Because digestate production and application costs were not measured directly in this study, the resulting economic balance should be interpreted as illustrative rather than as an experimentally validated net benefit.

Author Contributions

Conceptualization, I.V. and I.S.; methodology, K.S. and U.Ž.; software, I.V.; validation, I.V., K.S. and I.S.; formal analysis, I.S.; investigation, K.S.; resources, I.S.; data curation, I.V.; writing—original draft preparation, I.S.; writing—review and editing, U.Ž.; visualization, I.V. and I.S.; supervision, G.G.-Z. and I.V.; project administration, G.G.-Z. and I.S.; funding acquisition, I.S. All authors have read and agreed to the published version of the manuscript.

Funding

This research was supported by institutional research base funding from the Faculty of Agriculture and Food Technology, LBTU (project No. 14110-A03), and by the LBTU Doctoral Student Support and Development Initiative (ER36), grant No. 1.1.1.8/1/24/I/002, both of which contributed to the preparation of the manuscript, including analytical methods, interpretation of the results, and coverage of the Article Processing Charge (APC). Additional funding was provided by the project “Strengthening the Institutional Capacity of LBTU for Excellence in Studies and Research”, supported by the Recovery and Resilience Facility (ANM1), grant No. 5.2.1.1.i.0/2/24/I/CFLA/002, which covered data collection, experimental design, and the production of Furcellaria lumbricalis digestate through anaerobic digestion.

Data Availability Statement

The data that support the findings of this study are openly available at https://doi.org/10.71782/DATA/GFNEND.

Conflicts of Interest

The authors declare no conflicts of interest.

Appendix A

Table A1. Results of the redundancy analysis (RDA) permutation test. DF—degrees of freedom; F—pseudo-F statistic; pp-value. Asterisks (*) indicate statistically significant effects at p < 0.05. “Substrate” refers to the substrate type, and “Variant” refers to fertilizer and biostimulant treatment variants.
FactorDFVarianceFp
Substrate41,018,65155.550.001 *
Treatment557,9292.530.024 *
Table A2. Tukey pairwise comparisons between reduced fertilization treatments with biostimulant (F75_BIO3, F75_BIO6, F75_BIO12) and full mineral fertilization (F100_BIO0). SE—standard error; p-value—Tukey-adjusted significance level.
ComparisonEstimateSEp-Value
F75_BIO3–F100_BIO00.0450.1760.9998
F75_BIO6–F100_BIO00.1730.1760.9234
F75_BIO12–F100_BIO00.0370.1760.9999
Figure A1. Effect of biostimulant variants and substrate on total dry matter yield. Boxplots represent the distribution of yield values, with the median (line), interquartile range (box), and range (whiskers); points indicate individual observations. Colours indicate substrate type (Clay, ClayOM, Peat, Sand, SandOM). Treatments: F0_BIO0—no fertilizer; F100_BIO0—100% mineral fertilizer without biostimulant; F75_BIO0—75% mineral fertilizer without biostimulant; F75_BIO3, F75_BIO6, and F75_BIO12—75% mineral fertilizer combined with 3%, 6%, and 12% algal biostimulant, respectively.
Agronomy 16 00837 g0a1
Figure A2. Relationship between total dry matter yield (g m−2) and the first principal component (PC1), representing the nutrient availability gradient. Points represent individual observations, coloured according to substrate type (Clay, ClayOM, Peat, Sand, SandOM). The solid line indicates the fitted linear regression, and the shaded area represents the 95% confidence interval. The correlation coefficient (r = 0.27) and p-value (p = 0.0097) indicate a weak but statistically significant positive relationship.
Agronomy 16 00837 g0a2

References

  1. Arndt, C.; Diao, X.; Dorosh, P.; Pauw, K.; Thurlow, J. The Ukraine war and rising commodity prices: Implications for developing countries. Glob. Food Secur. 2023, 36, 100680. [Google Scholar] [CrossRef] [Scilit]
  2. Tandogan Aktepe, N.S.; Kayral, İ.E. Unraveling the Major Determinants behind Price Changes in Four Selected Representative Agricultural Products. Agriculture 2024, 14, 782. [Google Scholar] [CrossRef] [Scilit]
  3. Lin, F.; Li, X.; Jia, N.; Feng, F.; Huang, H.; Huang, J.; Fan, S.; Ciais, P.; Song, X.-P. The impact of Russia–Ukraine conflict on global food security. Glob. Food Secur. 2023, 36, 100661. [Google Scholar] [CrossRef] [Scilit]
  4. Guo, J.; Tanaka, T. Determinants of international price volatility transmissions: The role of self-sufficiency rates in wheat-importing countries. Humanit. Soc. Sci. Commun. 2019, 5, 124. [Google Scholar] [CrossRef] [Scilit]
  5. Tamasiga, P.; Ouassou, E.H.; Onyeaka, H.; Bakwena, M.; Happonen, A.; Molala, M. Forecasting disruptions in global food value chains to tackle food insecurity: The role of AI and big data analytics—A bibliometric and scientometric analysis. J. Agric. Food Res. 2023, 14, 100819. [Google Scholar] [CrossRef] [Scilit]
  6. Rouphael, Y.; Colla, G. Editorial: Biostimulants in agriculture. Front. Plant Sci. 2020, 11, 40. [Google Scholar] [CrossRef] [Scilit]
  7. Ali, O.; Ramsubhag, A.; Jayaraman, J. Biostimulant Properties of Seaweed Extracts in Plants: Implications towards Sustainable Crop Production. Plants 2021, 10, 531. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  8. Sani, M.N.H.; Yong, J.W.H. Harnessing Synergistic Biostimulatory Processes: A Plausible Approach for Enhanced Crop Growth and Resilience in Organic Farming. Biology 2022, 11, 41. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  9. Campobenedetto, C.; Mannino, G.; Beekwilder, J.; Contartese, V.; Karlova, R.; Bertea, C.M. The application of a biostimulant based on tannins affects root architecture and improves tolerance to salinity in tomato plants. Sci. Rep. 2021, 11, 354. [Google Scholar] [CrossRef] [Scilit]
  10. Sangha, J.S.; Kelloway, S.; Critchley, A.T.; Prithiviraj, B. Chapter seven—Seaweeds (macroalgae) and their extracts as contributors of plant productivity and quality: The current status of our understanding. In Advances in Botanical Research; Bourgougnon, N., Ed.; Academic Press: Cambridge, MA, USA, 2014; Volume 71, pp. 189–219. [Google Scholar] [CrossRef] [Scilit]
  11. Renaut, S.; Masse, J.; Norrie, J.P.; Blal, B.; Hijri, M. A commercial seaweed extract structured microbial communities associated with tomato and pepper roots and significantly increased crop yield. Microb. Biotechnol. 2019, 12, 1346–1358. [Google Scholar] [CrossRef] [Scilit]
  12. Mukherjee, A.; Patel, J.S. Seaweed extract: Biostimulator of plant defence and plant productivity. Int. J. Environ. Sci. Technol. 2019, 17, 553–558. [Google Scholar] [CrossRef] [Scilit]
  13. Raja, B.; Vidya, R. Application of seaweed extracts to mitigate biotic and abiotic stresses in plants. Physiol. Mol. Biol. Plants 2023, 29, 641–661. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  14. Pei, B.; Zhang, Y.; Liu, T.; Cao, J.; Ji, H.; Hu, Z.; Wu, X.; Wang, F.; Lu, Y.; Chen, N.; et al. Effects of seaweed fertilizer application on crops’ yield and quality in field conditions in China-A meta-analysis. PLoS ONE 2024, 19, e0307517. [Google Scholar] [CrossRef] [Scilit]
  15. Mannan, M.A.; Yasmin, A.; Sarker, U.; Bari, N.; Dola, D.B.; Higuchi, H.; Ercisli, S.; Ali, D.; Alarifi, S. Biostimulant red seaweed (Gracilaria tenuistipitata var. liui) extracts spray improves yield and drought tolerance in soybean. PeerJ 2023, 11, e15588. [Google Scholar] [CrossRef] [Scilit]
  16. Nivetha, N.; Shukla, P.S.; Nori, S.S.; Kumar, S.; Suryanarayan, S. A red seaweed Kappaphycus alvarezii-based biostimulant (AgroGain®) improves the growth of Zea mays and impacts agricultural sustainability by beneficially priming rhizosphere soil microbial community. Front. Microbiol. 2024, 15, 1330237. [Google Scholar] [CrossRef] [Scilit]
  17. Stirk, W.A.; Rengasamy, K.R.R.; Kulkarni, M.G.; Van Staden, J. Plant biostimulants from seaweed: An overview. In Plant Macronutrient Use Efficiency; Geisler, M., Giehl, R.F.H., Eds.; Academic Press: Cambridge, MA, USA, 2020; pp. 31–55. [Google Scholar] [CrossRef] [Scilit]
  18. González, A.; Castro, J.; Vera, J.; Moenne, A. Seaweed Oligosaccharides Stimulate Plant Growth by Enhancing Carbon and Nitrogen Assimilation, Basal Metabolism, and Cell Division. J. Plant Growth Regul. 2013, 32, 443–448. [Google Scholar] [CrossRef] [Scilit]
  19. Fuchs, W.; Drosg, B. Assessment of the state of the art of technologies for the processing of digestate residue from anaerobic digesters. Water Sci. Technol. 2013, 67, 1984–1993. [Google Scholar] [CrossRef] [Scilit]
  20. Nkoa, R. Agricultural benefits and environmental risks of soil fertilization with anaerobic digestates: A review. Agron. Sustain. Dev. 2014, 34, 473–492. [Google Scholar] [CrossRef] [Scilit]
  21. Dahiya, S.; Kumar, A.N.; Sravan, J.S.; Chatterjee, S.; Sarkar, O.; Venkata Mohan, S. Food waste biorefinery: Sustainable strategy for circular bioeconomy. Bioresour. Technol. 2018, 248, 2–12. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  22. Senevirathne, N.; Kaparaju, P. Enhancing the Agronomic Value of Anaerobic Digestate: A Review of Current vs. Emerging Technologies, Challenges and Future Directions. Agriculture 2025, 15, 2108. [Google Scholar] [CrossRef] [Scilit]
  23. Castellanos-Rozo, J.; Galvis, J.; Manjarres Hernández, E.; Merchán-Castellanos, M. Biosolids as fertilizer in the tomato crop. Rev. De La Fac. De Agron. De La Univ. Del Zulia 2022, 39, e223931. [Google Scholar] [CrossRef] [Scilit]
  24. Jensen, L.S.; Schjoerring, J.K.; van der Hoek, K.W.; Poulsen, H.D.; Zevenbergen, J.F.; Pallière, C.; Lammel, J.; Brentrup, F.; Jongbloed, A.W.; Willems, J.; et al. Benefits of nitrogen for food, fibre and industrial production. In The European Nitrogen Assessment; Sutton, M.A., Howard, C.M., Erisman, J.W., Eds.; Cambridge University Press: Cambridge, MA, USA, 2011; pp. 32–61. [Google Scholar] [CrossRef] [Scilit]
  25. Jankauskienė, J.; Laužikė, K.; Kaupaitė, S. The Use of Anaerobic Digestate for Greenhouse Horticulture. Agronomy 2024, 14, 2437. [Google Scholar] [CrossRef] [Scilit]
  26. Zodape, S.T.; Mukhopadhyay, S.; Eswaran, K.; Reddy, M.; Chikara, J. Enhanced yield and nutritional quality in green gram (Phaseolus radiata L.) treated with seaweed (Kappaphycus alvarezii) extract. J. Sci. Ind. Res. 2010, 69, 468–471. [Google Scholar]
  27. FitzGerald, J.A.; Allen, E.; Wall, D.M.; Jackson, S.A.; Murphy, J.D.; Dobson, A.D. Methanosarcina Play an Important Role in Anaerobic Co-Digestion of the Seaweed Ulva lactuca: Taxonomy and Predicted Metabolism of Functional Microbial Communities. PLoS ONE 2015, 10, e0142603. [Google Scholar] [CrossRef] [Scilit]
  28. Adams, J.M.M.; Toop, T.A.; Donnison, I.S.; Gallagher, J.A. Seasonal variation in Laminaria digitata and its impact on biochemical conversion routes to biofuels. Bioresour. Technol. 2011, 102, 9976–9984. [Google Scholar] [CrossRef] [Scilit]
  29. Barbot, Y.N.; Al-Ghaili, H.; Benz, R. A Review on the Valorization of Macroalgal Wastes for Biomethane Production. Mar. Drugs 2016, 14, 120. [Google Scholar] [CrossRef] [Scilit]
  30. Jard, G.; Marfaing, H.; Carrère, H.; Delgenes, J.-P.; Steyer, J.-P.; Dumas, C. French Brittany macroalgae screening: Composition and methane potential for potential alternative sources of energy and products. Bioresour. Technol. 2013, 144, 492–498. [Google Scholar] [CrossRef] [Scilit]
  31. Philp, J.C.; Ritchie, R.J.; Allan, J.E. Biobased chemicals: The convergence of green chemistry with industrial biotechnology. Trends Biotechnol. 2013, 31, 219–222. [Google Scholar] [CrossRef] [Scilit]
  32. Stegmann, P.; Londo, M.; Junginger, M. The circular bioeconomy: Its elements and role in European bioeconomy clusters. Resour. Conserv. Recycl. X 2020, 6, 100029. [Google Scholar] [CrossRef] [Scilit]
  33. Yaashikaa, P.R.; Kumar, P.S.; Varjani, S.; Saravanan, A. A critical review on the biochar production techniques, characterization, stability and applications for circular bioeconomy. Biotechnol. Rep. 2020, 28, e00570. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  34. Alvarado-Morales, M.; Boldrin, A.; Karakashev, D.B.; Holdt, S.L.; Angelidaki, I.; Astrup, T. Life cycle assessment of biofuel production from brown seaweed in Nordic conditions. Bioresour. Technol. 2013, 129, 92–99. [Google Scholar] [CrossRef] [Scilit]
  35. Seghetta, M.; Tørring, D.; Bruhn, A.; Thomsen, M. Bioextraction potential of seaweed in Denmark—An instrument for circular nutrient management. Sci. Total Environ. 2016, 563–564, 513–529. [Google Scholar] [CrossRef] [Scilit]
  36. Seghetta, M.; Romeo, D.; D’Este, M.; Alvarado-Morales, M.; Angelidaki, I.; Bastianoni, S.; Thomsen, M. Seaweed as innovative feedstock for energy and feed—Evaluating the impacts through a life cycle assessment. J. Clean. Prod. 2017, 150, 1–15. [Google Scholar] [CrossRef] [Scilit]
  37. Farghali, M.; Mohamed, I.M.A.; Osman, A.I.; Rooney, D.W. Seaweed for climate mitigation, wastewater treatment, bioenergy, bioplastic, biochar, food, pharmaceuticals, and cosmetics: A review. Environ. Chem. Lett. 2023, 21, 97–152. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  38. Skapste, I.; Vircava, I.; Skutele, K.; Žaimis, U.; Grinberga-Zalite, G.; Zvirbule, A. Algae digestate biostimulants as an innovative solution for food system sustainability and productivity improvement. Front. Sustain. Food Syst. 2025, 9, 1656867. [Google Scholar] [CrossRef] [Scilit]
  39. Skapste, I.; Balina, K.; Zaimis, U.; Grinberga-Zalite, G.; Zvirbule, A. Life cycle assessment of Furcellaria lumbricalis biostimulant production: Towards a circular bioeconomy in the Baltic Sea region. In Proceedings of the 33rd European Biomass Conference and Exhibition (EUBCE 2025), Valencia, Spain, 9–12 June 2025. [Google Scholar]
  40. ISO 10390:2005; Soil Quality—Determination of pH. International Organization for Standardization: Geneva, Switzerland, 2005.
  41. ISO 10694:1995; Soil Quality—Determination of Organic and Total Carbon After Dry Combustion (Elementary Analysis). International Organization for Standardization: Geneva, Switzerland, 1995.
  42. ISO 13878:1998; Soil Quality—Determination of Total Nitrogen Content by Dry Combustion (“Elemental Analysis”). International Organization for Standardization: Geneva, Switzerland, 1998.
  43. ISO 11277:2009; Soil quality—Determination of Particle Size Distribution in Mineral Soil Material—Method by Sieving and Sedimentation. International Organization for Standardization: Geneva, Switzerland, 2009.
  44. Skapste, I.; Grinberga-Zalite, G.; Žaimis, U. Economic Potential of Algae Biostimulant for Sustainable Agriculture in the Baltic Sea Region: Impact of Furcellaria lumbricalis Digestate Extract on Basil Growth Promotion. Sustainability 2025, 17, 3268. [Google Scholar] [CrossRef] [Scilit]
  45. Amadou, A.; Song, A.; Tang, Z.-X.; Li, Y.; Wang, E.-Z.; Lu, Y.-Q.; Liu, X.-D.; Yi, K.; Zhang, B.; Fan, F. The Effects of Organic and Mineral Fertilization on Soil Enzyme Activities and Bacterial Community in the Below- and Above-Ground Parts of Wheat. Agronomy 2020, 10, 1452. [Google Scholar] [CrossRef] [Scilit]
  46. Tamagno, S.; McClellan Maaz, T.; van Kessel, C.; Linquist, B.A.; Ladha, J.K.; Lundy, M.E.; Maureira, F.; Pittelkow, C.M. Critical assessment of nitrogen use efficiency indicators: Bridging new and old paradigms to improve sustainable nitrogen management. Eur. J. Agron. 2024, 159, 127231. [Google Scholar] [CrossRef] [Scilit]
  47. Romio, C.; Ward, A.J.; Møller, H.B. Characterization and valorization of biogas digestate and derived organic fertilizer products from separation processes. Front. Sustain. Food Syst. 2024, 8, 1415508. [Google Scholar] [CrossRef] [Scilit]
  48. Kārkliņš, A.; Alpiņa, I. Fertilization Recommendations for Vegetables in Latvia [Advisory Material]; Latvia University of Life Sciences and Technologies: Jelgava, Latvia, 2018. [Google Scholar]
  49. Mannino, G.; Ricciardi, M.; Gatti, N.; Serio, G.; Vigliante, I.; Contartese, V.; Gentile, C.; Bertea, C.M. Changes in the Phytochemical Profile and Antioxidant Properties of Prunus persica Fruits after the Application of a Commercial Biostimulant Based on Seaweed and Yeast Extract. Int. J. Mol. Sci. 2022, 23, 15911. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  50. Hughes, A.D.; Kelly, M.S.; Black, K.D.; Stanley, M.S. Biogas from Macroalgae: Is it time to revisit the idea? Biotechnol. Biofuels 2012, 5, 86. [Google Scholar] [CrossRef] [Scilit]
  51. Milledge, J.J.; Harvey, P.J. Potential process ‘hurdles’ in the use of macroalgae as feedstock for biofuel production in the British Isles. J. Chem. Technol. Biotechnol. 2016, 91, 2211–2231. [Google Scholar] [CrossRef] [Scilit]
  52. Hossen, I.; Saha, R.; Bhuiya, M.; Hoque, N.M.M. Third-generation biodiesel development in Bangladesh: A review of recent trends, prospects, and economic analysis. Future Energy 2025, 4, 48–58. [Google Scholar] [CrossRef] [Scilit]
  53. Li, J.; Van Gerrewey, T.; Geelen, D. A meta-analysis of biostimulant yield effectiveness in field trials. Front. Plant Sci. 2022, 13, 836702. [Google Scholar] [CrossRef] [Scilit]
  54. Kulkarni, M.G.; Rengasamy, K.R.R.; Pendota, S.C.; Gruz, J.; Plačková, L.; Novák, O.; Doležal, K.; Van Staden, J. Bioactive molecules derived from smoke and seaweed Ecklonia maxima showing phytohormone-like activity in Spinacia oleracea L. New Biotechnol. 2019, 48, 83–89. [Google Scholar] [CrossRef] [Scilit]
  55. La Bella, S.; Consentino, B.B.; Rouphael, Y.; Ntatsi, G.; De Pasquale, C.; Iapichino, G.; Sabatino, L. Impact of Ecklonia maxima Seaweed Extract and Mo Foliar Treatments on Biofortification, Spinach Yield, Quality and NUE. Plants 2021, 10, 1139. [Google Scholar] [CrossRef] [Scilit]
  56. Sutherland, A.D.; Varela, J.C. Comparison of various microbial inocula for the efficient anaerobic digestion of Laminaria hyperborea. BMC Biotechnol. 2014, 14, 7. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  57. Jolliffe, I.T.; Cadima, J. Principal component analysis: A review and recent developments. Philos. Trans. Ser. A Math. Phys. Eng. Sci. 2016, 374, 20150202. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  58. Legendre, P.; Legendre, L. Chapter 11—Canonical analysis. In Developments in Environmental Modelling; Legendre, P., Legendre, L., Eds.; Elsevier: Amsterdam, The Netherlands, 2012; Volume 24, pp. 625–710. [Google Scholar] [CrossRef] [Scilit]
  59. Diacono, M.; Montemurro, F. Long-term effects of organic amendments on soil fertility. A review. Agron. Sustain. Dev. 2010, 30, 401–422. [Google Scholar] [CrossRef] [Scilit]
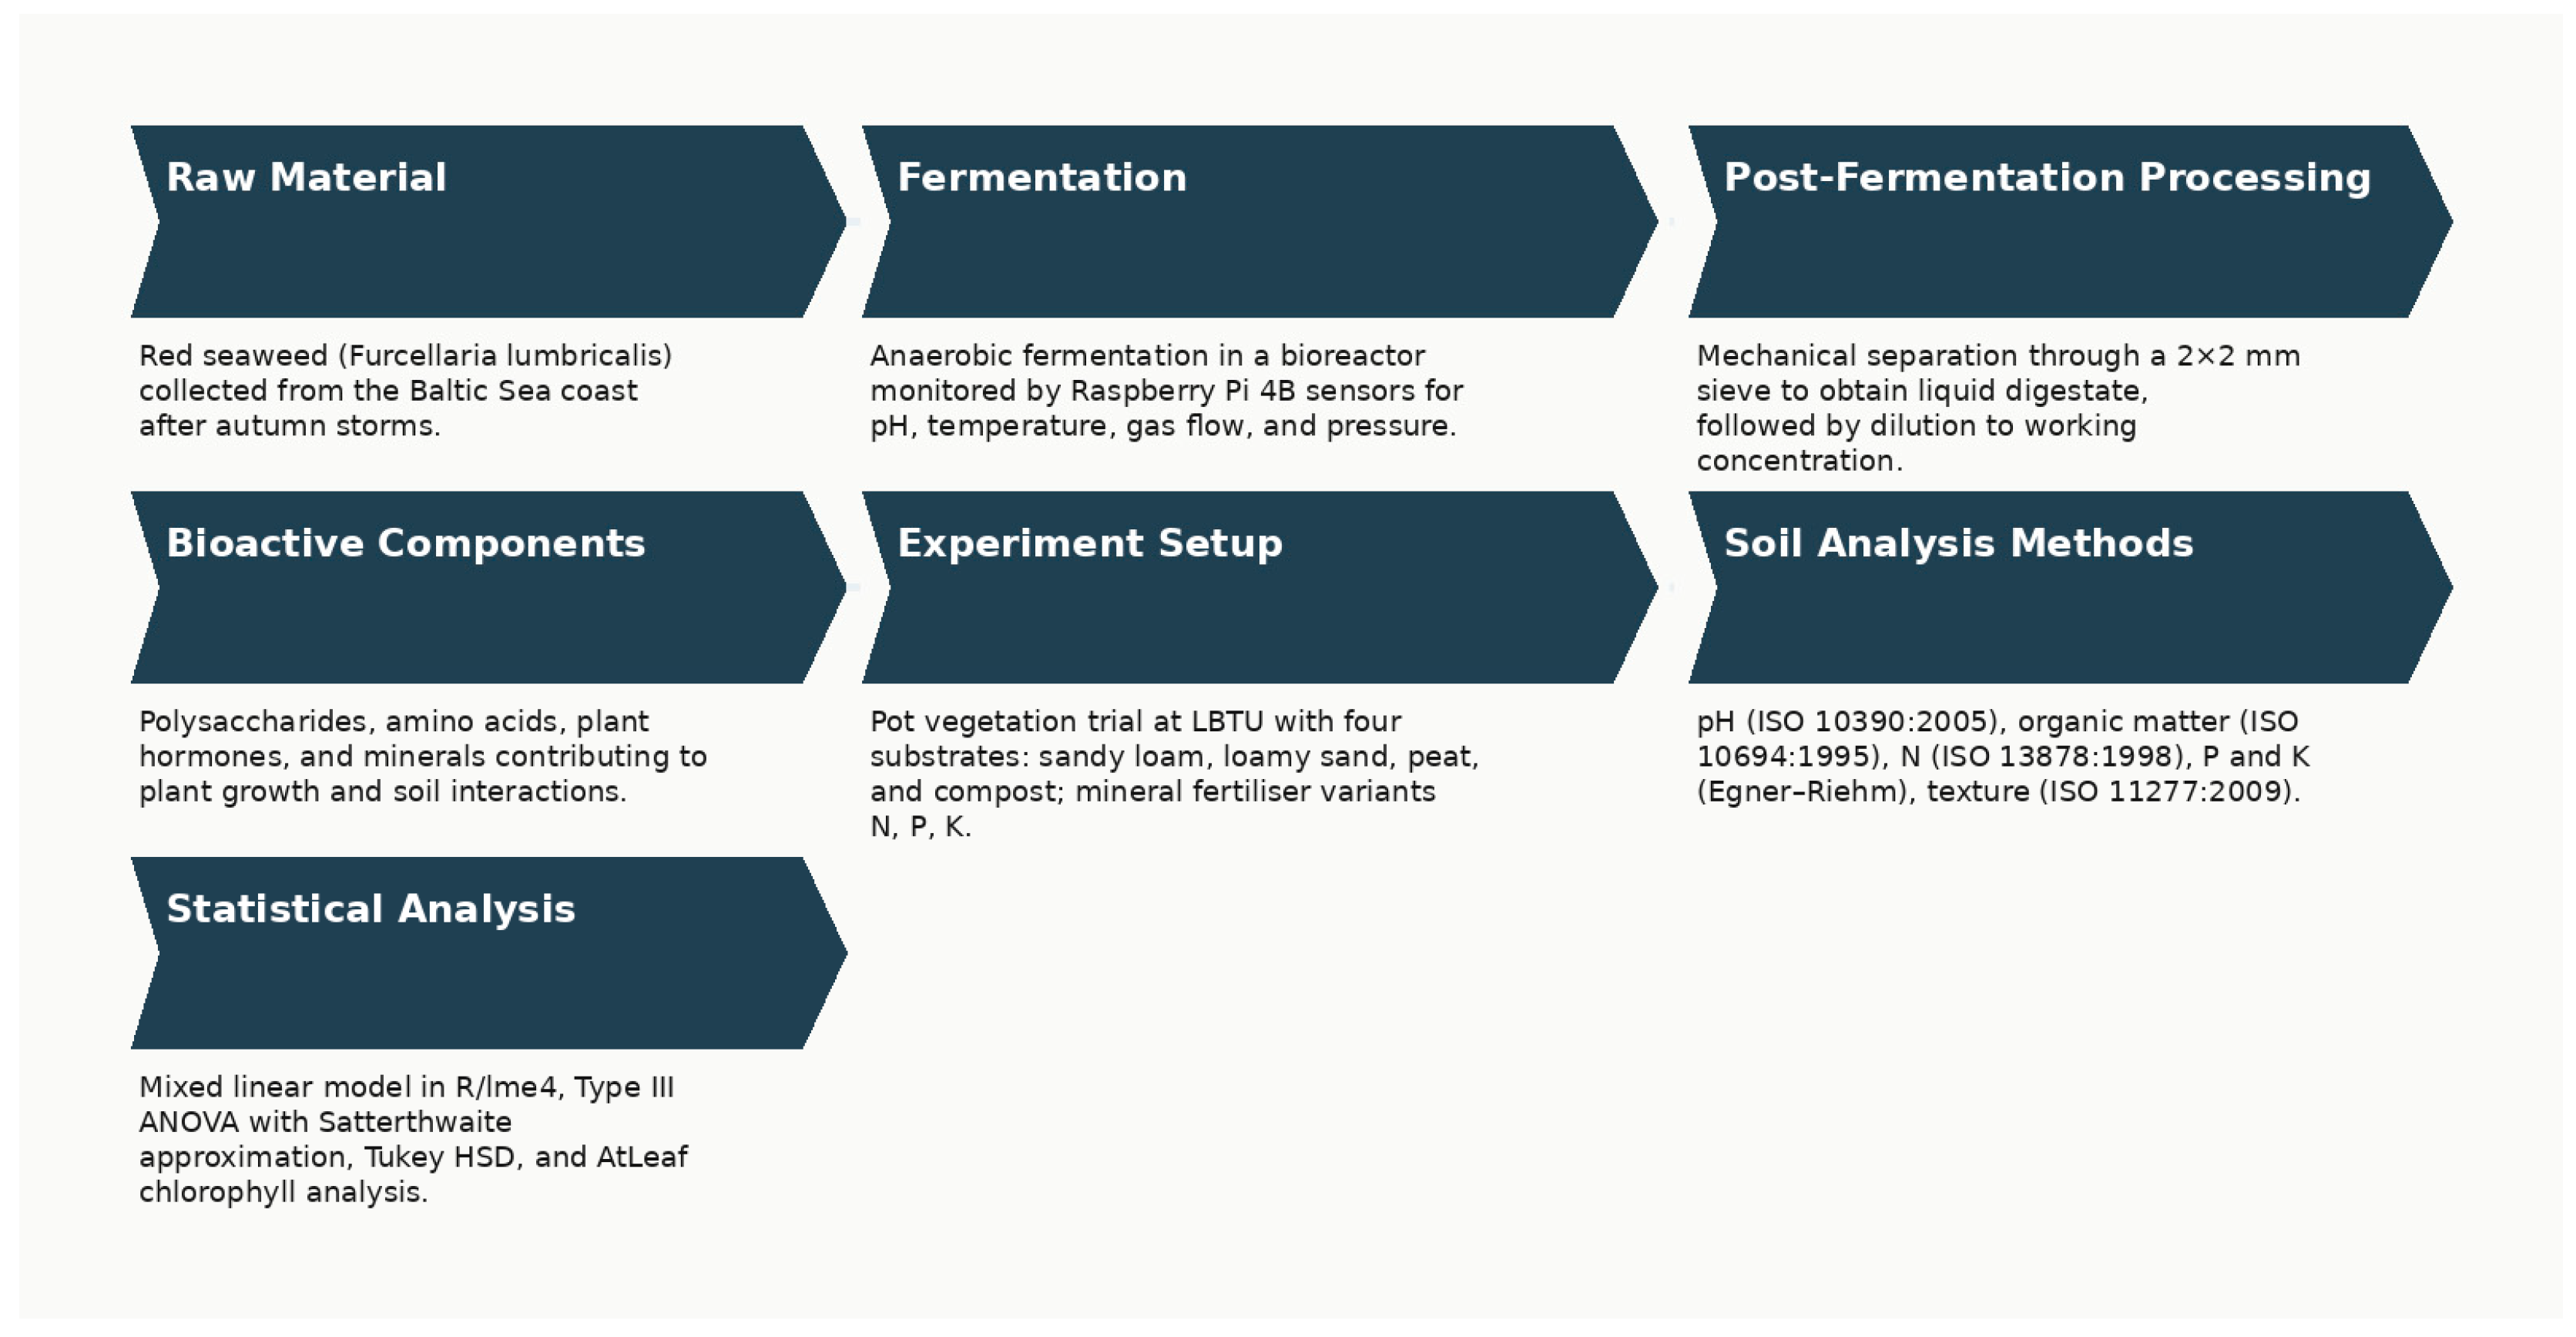
Figure 1. Overview of the experimental design, from Furcellaria lumbricalis digestate production through pot trials in contrasting substrates to multivariate data analysis (PCA/RDA and ANOVA). Soil chemical analyses were performed according to ISO 10390:2005 [40], ISO 10694:1995 [41], ISO 13878:1998 [42], and ISO 11277:2009 [43].
Agronomy 16 00837 g001
Figure 2. Effect of biostimulant treatments on the modeled total dry matter yield (g m−2) across different substrates. Points represent estimated marginal means (emmeans) from the linear mixed model, and error bars indicate 95% confidence intervals (Cl). Treatments: F0_BIO0—no fertilizer; F100_BIO0—100% mineral fertilizer without biostimulant; F75_BIO0—75% mineral fertilizer without biostimulant; F75_BIO3, F75_BIO6, and F75_BIO12—75% mineral fertilizer combined with 3%, 6%, and 12% algal biostimulant, respectively.
Agronomy 16 00837 g002
Figure 3. Principal component analysis (PCA) for chemical and biological parameters of substrates. The arrows represent the direction and strength of variable contributions (pH (KCl), P2O5, K2O, AtLeaf (leaf chlorophyll index), MBA (microbial biomass activity)) to the principal components. The points are colored according to substrate type (Cla, ClayOM, Peat, Sand, and SandOM) and symbols indicate fertilizer and biostimulant treatments (F0_BIO0, F100_BIO0, F75_BIO0, F75_BIO3, F75_BIO6, and F75_BIO12). Percentages on the axes indicate the proportion of explained variance.
Agronomy 16 00837 g003
Figure 4. Redundancy analysis (RDA) of substrate and biostimulant effects on the measured chemical and biological parameters. The points represent individual samples, colored according to substrate type (Clay, ClayOM, Peat, Sand, and SandOM). The ellipses indicate group dispersion for each substrate. The percentages on the axes represent the proportion of variance explained by each RDA.
Agronomy 16 00837 g004
Table 1. Chemical properties of substrates. Organic matter content, soil reaction (based on pH KCl), and available phosphorus (P2O5) and potassium (K2O) levels are presented. Qualitative classes (e.g., insufficient, optimal, and high) indicate substrate suitability for plant growth according to standard agronomic evaluation criteria. N/A—not applicable.
SubstrateOrganic Matter (%) Organic Matter ContentpH KClSoil ReactionP2O5, mg kg−1Available P2O5 Content in Soil/SubstrateK2O, mg kg−1Available K2O Content in Soil/Substrate
Sandy clay with organic matter (ClayOM)5.1Promoted7.0Normal240High262Medium
Sandy clay (Clay)2.1Insufficient7.1Normal28Very low99Low
Sands containing organic matter (SandOM)1.7Optimal6.1Normal125High64Medium
Sand0.6Insufficient5.6Normal26Low130High
Peat99.0N/A5.0Normal215Low1270Very high
Table 2. Mineral fertilizer rates (N, P2O5, and K2O) applied in different substrates and treatment variants of the pot experiment. Fertilizer rate was expressed as a percentage of the full mineral fertilizer dose. Treatments: F0_BIO0—no fertilizer; F100_BIO0—100% mineral fertilizer without biostimulant; F75_BIO0—75% mineral fertilizer without biostimulant; F75_BIO3, F75_BIO6, and F75_BIO12—75% mineral fertilizer combined with 3%, 6%, and 12% algal biostimulant, respectively. Nutrient amounts were expressed as mg L−1 for peat and kg ha−1 for mineral substrates (Clay, ClayOM, Sand, and SandOM).
SubstrateVariantFertilizer Rate, %NP2O5K2O
Clay, ClayOM, Peat, Sand, SandOMF0_BIO00000
PeatF100_BIO0100185185462
PeatF75_BIO075138138346
PeatF75_BIO3/6/1275138138346
ClayF100_BIO010080100120
ClayF75_BIO075607590
ClayF75_BIO3/6/1275607590
ClayOMF100_BIO01006050100
ClayOMF75_BIO075453875
ClayOMF75_BIO3/6/1275453875
SandF100_BIO010080100100
SandF75_BIO075607575
SandF75_BIO3/6/1275607575
SandOMF100_BIO01006050120
SandOMF75_BIO075453890
SandOMF75_BIO3/6/1275453890
Note: Peat substrate quantities in mg L−1; mineral substrates (Clay, ClayOM, Sand, SandOM) kg ha−1.
Table 3. Dunnett contrasts with the control (model without interaction). Δ harvest indicates the difference in total dry matter yield compared to the control treatment (F0_BIO0). SE—standard error; p—significance level. Treatments: F0_BIO0—no fertilizer; F100_BIO0—100% mineral fertilizer without biostimulant; F75_BIO0—75% mineral fertilizer without biostimulant; F75_BIO3, F75_BIO6, and F75_BIO12—75% mineral fertilizer combined with 3%, 6%, and 12% algal biostimulant, respectively.
Contrast (vs. F0_BIO0)Δ HarvestSEp
F100_BIO0+0.71400.1760.0016
F75_BIO0+0.62470.1760.0085
F75_BIO12+0.67670.1760.0033
F75_BIO3+0.66870.1760.0038
F75_BIO6+0.54130.1760.0337
Table 4. Estimation of mineral fertilizer costs and conceptual economic assessment for the 75% NPK + biostimulant scenario. Typical nutrient application rates and market prices were used to estimate mineral fertilizer costs for radish cultivation. The net economic effect represents the difference between reduced fertilizer costs under the 75% NPK scenario and the estimated digestate costs. NPK—nitrogen (N), phosphorus (P2O5) and potassium (K2O). All values are expressed per hectare (ha−1); prices are expressed in EUR t−1.
ParameterValueNotes/Source
Typical dose of N for radishes100–150 kg N ha−1[48]
Typical dose of P2O5 for radishes80–120 kg P2O5 ha−1[48]
Typical dose of K2O for radishes120–180 kg K2O ha−1[48]
N price600 EUR t−1[4,13]
P2O5 price550 EUR t−1[4,13]
K2O price480 EUR t−1[4,13]
Calculated costs
100% NPK costEUR 162–242 ha−1(N dose × 0.6) + (P2O5 dose × 0.55) + (K2O dose × 0.48)
75% NPK costEUR 121–182 ha−1100% NPK cost × 0.75
Estimated fertilizer cost savingsEUR 40–61 ha−1100% NPK costs—75% NPK costs
Digestate costs (conceptual interval)
Costs of the digestate of Furcellaria lumbricalisEUR 20–30 ha−1[1,49]
Net economic balance
Net economic effectEUR 10–41 ha−1[15]
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.