


Abstract
The non-essential metalloid arsenic (As) is widely distributed in soil and underground water of many countries. Arsenic contamination is a concern because it creates threat to food security in terms of crop productivity and food safety. Plants exposed to As show morpho-physiological, growth and developmental disorder which altogether result in loss of productivity. At physiological level, As-induced altered biochemistry in chloroplast, mitochondria, peroxisome, endoplasmic reticulum, cell wall, plasma membrane causes reactive oxygen species (ROS) overgeneration which damage cell through disintegrating the structure of lipids, proteins, and DNA. Therefore, plants tolerance to ROS-induced oxidative stress is a vital strategy for enhancing As tolerance in plants. Plants having enhanced antioxidant defense system show greater tolerance to As toxicity. Depending upon plant diversity (As hyperaccumulator/non-hyperaccumulator or As tolerant/susceptible) the mechanisms of As accumulation, absorption or toxicity response may differ. There can be various crop management practices such as exogenous application of nutrients, hormones, antioxidants, osmolytes, signaling molecules, different chelating agents, microbial inoculants, organic amendments etc. can be effective against As toxicity in plants. There is information gap in understanding the mechanism of As-induced response (damage or tolerance response) in plants. This review presents the mechanism of As uptake and accumulation in plants, physiological responses under As stress, As-induced ROS generation and antioxidant defense system response, various approaches for enhancing As tolerance in plants from the available literatures which will make understanding the to date knowledge, knowledge gap and future guideline to be worked out for the development of As tolerant plant cultivars.
1. Introduction
Arsenic (As) is an environmental non-essential metalloid that poses a severe risk to all forms of plant and animal life [1,2]. It is a naturally occurring 20th most plentiful and widely distributed element on the planet. At present, more than 2.5 billion people on the earth depend on groundwater, and contamination of groundwater by As-tainted toxicity has become a serious concern [3]. Contamination of As in groundwater is increasing daily and it is estimated that 500 million people round the globe will be affected by As contamination. This metalloid enters into the ecosystem via natural activities such as weathering and mineralization of earth crust and also by anthropogenic activities that include application of As-based pesticides, insecticides, fertilization with municipal solid wastes, and irrigation with As-tainted groundwater [4]. Thus, animals and humans are irradiated to As directly through the consumption of As-tainted water or indirectly by ingestion of foods from the ecosystem. It is well-known that food chain is affected by As when agricultural products become contaminated [5].
Plants exhibit morphological and physio-biochemical disorders due to As toxicity. It has been reported that root proliferation and extension are inhibited by As because root is the foremost organ to be subjected to As [6]. Arsenic contamination reduces nodule formation in roots and shows wilting, curling, and necrosis of leaf blades. Arsenic toxicity hampers plant growth by decreasing cell proliferation and biomass buildup. Arsenic binds to enzymes and proteins, impairing cell biochemistry and disrupting physiological processes like photosynthesis, respiration, transpiration in plants [4]. It can deplete plants reproductive capacity, obstructing photosynthetic processes and resulting in decreased plant growth and yield [7,8].
Reactive oxygen species (ROS) are continuously evolved by plants under stress conditions and generate oxidative stress which adversely affects different cell components like lipids, proteins, and DNA [9,10]. Higher level of As(III) and As(V) exposure promotes the accumulation of ROS in plants and those play role in the translation of As(V) into As(III) [11,12]. Arsenic toxicity enhances lipid peroxidation that damages cellular membranes by electrolyte leakage (El, [13]).
Plant continuously fostered robust machineries to fight against injurious effects of ROS by using enzymatic antioxidants including, superoxide dismutase (SOD), catalase (CAT), ascorbate peroxidase (APX), glutathione reductase (GR), monodehydroascorbate reductase (MDHAR), dehydroascorbate reductase (DHAR), glutathione peroxidase (GPX), glutathione S-transferase (GST), and non-enzymatic antioxidants including, ascorbic acid (AsA), glutathione (GSH), tocopherol, phenolic acids, carotenoids, non-protein amino acids etc. Antioxidant enzyme activities are key players for scavenging ROS directly or indirectly from stressed cells [14]. A steady-state balance is maintained in plant cells, the antioxidant defense system, and ROS buildup. Besides, an optimal ROS level in the plant cells allows for appropriate redox biology reactions and aid in the adjustment of variety of activities required for plant growth progressions [10,15,16]. Literature describes that As stress directs to oxidative stress and promotes functions of antioxidant enzyme to counteract this stress in rice [17,18].
Although many reports are available on the mechanisms of As accumulation, absorption, and toxicity in plants, the information regarding As-provoked oxidative stress and antioxidant defense mechanisms are still inadequately recognized in plants. Therefore, this article discusses the mechanisms of As-induced oxidative stress and the involvement of antioxidant defense systems in detoxification of As-stimulated oxidative injury in plants.
2. Arsenic Uptake and Accumulation in Plants
In soil, organic As compounds remain in addition to inorganic As. The inorganic and organic both forms of As in soil can be uptaken by plants while the higher rate and part is the inorganic As. Arsenate [As(V)]/AsO43− and arsenite [As(III)]/AsO33− are the inorganic entities. Generally inorganic forms, As(III) and As(V) are more toxic than the organic form. Aerobic soil predominates the generation of As(V) and anaerobic/inundated soil is predominated by the occurrence of As(III) [19]. Methylated As [monomethylarsinic acid (CH3AsO(OH)2; MMA) along with dimethylarsinic acid ((CH3)2AsOOH); DMA)] are commonly demonstrated organic As compound. Microorganisms are involved in conversion of As(V)/As(III) to MMA and DMA by distinct pathway. It is very usual that root is the first organ through which As enters the plants but As can enter through all the submerged parts of plants [20]. After crossing the root epidermis and passing through the apoplastic and symplastic pathways, As enters the xylem or phloem through which bulk flow of As occurs and can be distributed to different plant organs including stem, leaf, reproductive parts and even seeds. However, cell wall, especially the membrane plays pivotal responsibility for controlling the rate and amount of As transport though it is variable among As accumulators and non-accumulators. Plant’s root/membrane selective transporters and pathways are concerned for the entrance, uptake and translocation of inorganic and organic As [21]. A schematic illustration of As uptake and accumulation in plants has been presented in Figure 1.
Figure 1.
Schematic illustration of As uptake, translocation, accumulation and detoxification in plants. The dotted arrows indicate that the pathways/mechanism are not known properly. MMA: monomethylarsinic acid [(CH3AsO(OH)2)]; DMA: dimethylarsinic acid [(CH3)2AsOOH)]; nodulin 26-like intrinsic proteins (NIPs)) which are as a group recognized as aquaporin channels (AQPs: OsNIP); OsPHT: phosphate transporter; PIPs: plasma membrane intrinsic proteins (OsPIP); OsABCC1: C type ATP-binding cassette transporter; OsPTR7: putative peptide transporter; AtINT: inositol transporters; AR: As (V) reductase. As (V) can be entered to the root through OsPHT. As (III) can be entered or to be excreted through AQPs/OsNIP. As (V) can be converted into As (III) by the activity of AR. As (III) can be bound to GSH to form PCs complex and sequestrated into vacuole. As (III) can also converted into organic DMA and MMA (but the mechanism is not known clearly), both of the organic forms can be excreted outside the cell through unknown transporter. DMA and MMA can also enter the cell trough AQPs/OsNIP. The AQPs/OsNIP, OsPHT and OsPTR7 have been assumed to be the transporter of various As species [As(III)/As(V)/MMA/DMA] towards the shoot and grain. Some of the As can also be released to the atmosphere as volatile As compounds.
Arsenite [As(III)/AsO33−] mainly enters through the root nodulin 26-like intrinsic proteins (NIPs) and these are as a group recognized as aquaporin channels (AQPs) in together. Expression of OsNIP2;1 (Lsi1), in rice (Oryza sativa) root were reported in distant part of the plasma membrane in the zone of Casparian strips. OsNIP2;1 (Lsi1) regulates the influx of silicic acid (Si(OH)4) and As(III) [22]. Another aquaporin channel OsNIP2;2 (Lsi2) is also found in plasma membrane of cells in both exodermis and endodermis of O. sativa root. These are Si(OH)4 efflux transporters. Here, Lsi2 is restricted to the proximal side cell [23]. Influx of Si(OH)4) as well as As(III) occur through Lsi1 whereas efflux of Si(OH)4 occur through Lsi2; this process hinders As(III) entrance [22]. As(III) entrance in a number of plant species is bi-directional and is regulated by concentration difference. Similar mechanism was noticed in different plants like Pteris vittata, Lotus japonicas and Arabidopsis thaliana [24,25,26].
Plasma membrane intrinsic proteins (PIPs), such as OsPIP2;4, OsPIP2;6 and OsPIP2;7 can also control As(III) entrance but the mechanism is still ambiguous [27]. When As is present attaching the root zone, it can enter the root or efflux from the root or because of its affinity it can be bound to GSH as well as its derivatives phytochelatins (PCs) [28]. Once forming the As(III)-PCs it is sequestrated in vacuole mediated by C-type ATP-binding cassette transporter (OsABCC1) [29].
Arsenate [As(V)]/AsO43− is the most common form of As under aerobic and dry condition and structurally it is resembled to PO43−; this is the cause for using the same transporter/pathway by both species [21]. PO43− transporter genes (OsPHTs) were recognized and phosphate transporter, OsPHT1;8 (OsPT8) and OsPHT1;1 showed high affinity for PO43− and As(V) in O. sativa L. [30]. However, after uptaking As(V), it is quickly converted into As(III) where As(V) reductase (AR) activity is involved. There are two As (V) reductases, OsHAC1;1 and OsHAC1;2 in the root of O. sativa [31]. This converted As (III) can be released outside of the root through efflux or it can be converted into As(III)-PC complexes; mechanism of the both has been discussed in the previous part of this section.
Aquaporin Lsi1 has been proposed to be involved in entrance of MMA(V) as well as DMA(V) in O. sativa [32]. So, Lsi1 is involved in both the inorganic As (III) in addition to organic As transportation. Occurrence of MMA(V)-thiol complexes were also documented [33] whereas little is known about DMA(V) and it needs further study.
Arsenic transfer from root to other vegetative parts and to reproductive parts has been studied, moreover described in few reports which are mostly on O. sativa L. As(III) is more quickly taken up by root than the other organic species of As. OsNIP2;1 (Lsi1) is accountable for As(III) entrance, and Lsi2 is for As(III) efflux from root to xylem as reported in O. sativa L. [34]. Lsi1 and Lsi2 work sequentially or together for controlling the root entrance of Si along with As(III). Besides, Lsi1, Lsi2 and Lsi6 transpiration pool is also vital to manage As uptake [35]. In O. sativa, various Pi transporter genes (OsPT) have been reported which transport P and As(V) towards the root; some of which are OsPT1, OsPT2, OsPT4, OsPT6 [36]. AsV in converted to As(III) within root, after that it can enter the xylem via Lsi 2 [37]. The organic DMA as well as MMA cross aquaporin channels [38]. The DMA is tremendously mobile all through the vascular tissues; it can be transported very quickly from root to shoot and from leaves to seed in O. sativa. In O. sativa L. grain, As(III) is mainly translocated via phloem whereas DMA is translocated via both kinds of vascular tissues. A putative peptide transporter, OsPTR7 functions for in the long-distance transportation and accumulation of DMA [39]. Also, inositol transporters, AtINT2 and AtINT4 may function for the entrance of As(III) to phloem and its translocation into grain.
3. Arsenic Toxicity in Plants
Many studies reported that As availability in the soil can hamper the morphological and physio-biochemical functioning of plants consequently reducing crop yield (Figure 2); [2,40,41,42]. For instance, plants exposed to As showed discoloration, lignification, and plasmolysis of root cells which resulted in stunted plant growth [43]. In addition, As contamination severely reduced germination percentage, shoot and root elongation, root and leaf biomass, and seed vigor index of different plants [44,45,46]. Likewise, As exposure has been shown to reduce the leaf numbers, area of leaf, height of plant, and fresh and dry biomass of plants [47,48]. Reduced biomass in the presence of As was possibly an outcome of enhanced permeability of the cell membranes, consequently increased leakage of cellular constituents/basic nutrients essentially required for energy generation, and optimum growth and development of plants [49].
Figure 2.
Arsenic-induced morphological and physiological responses of plants.
Arsenic stress regulates water relation in plants [1,50]. For example, As stress reduced relative water content in wheat and pea plants [51,52]. Likewise, As stress in lettuce reduced water use efficiency (WUE), stomatal conductance, and increased plant transpiration rate [53]. In Hydrilla verticillata, As exposure reduced WUE and increased transpiration rate [54]. The As stress may disrupt the cell wall structure in leaves, resulting in decreased leaf water content.
Many studies described that As stress inhibited the activities of photosynthetic machineries in plants [50,55]. Arsenic toxicity causes decrease in the synthesis of photosynthetic pigments, distortion of chloroplast, and reduction of photosystem I (PSI) and photosystem II (PSII) activities [56]. Several plants such as Zea mays, Trifolium pratense, and Lactuca sativa decreased biosynthesis of chlorophyll (Chl) due to As stress [57,58,59]. In chickpea (Cicer arietinum) plants, As toxicity reduced Chl contents and consequently resulted in chloroplast distortion [60]. In soybean, As stress reduced the efficacy of PSII, stomatal conductance, and rate of photosynthesis [61]. Arsenic stress reduced Chl fluorescence and photosynthetic rate in P. cretica and Spinacia oleracea [42]. Arsenic-induced reduction in Chl content may be due to the reduction in ribulose-1,5-bisphosphate carboxylase/oxygenase (RuBisCO) activity and degrading biosynthetic enzymes, δ-aminolevulinic acid dehydratase and protochlorophyllide reductase [62]. It has been reported that As toxicity initiates disruption of microtubules that hampers the formation of stomata which results in abnormal stomata [63]. Arsenic stress triggers phosphatidic acid (PA) signaling and that PA involved in stomatal closure of soybean [64]. Arsenic-induced injurious effects on roots may affect the uptake of water and ions, which consequently, reduces the photosynthetic and transpiration rate and inhibits stomatal regulation [65,66].
Arsenic toxicity damages cell membranes and it is well-known that chloroplast membranes are quite sensitive to As-induced damages [2]. Arsenic-stressed P. vittata and Leucaena leucocephala leaves showed abnormal internal membranes of chloroplasts [67,68]. Literature shows that As stress led to perturbations in the chloroplast membranes organizations such as thylakoid membrane rupture and swelling [5]. In addition, Upadhyaya et al. [69] reported that As toxicity distorted chloroplast membrane and reduced carotenoids. Arsenic toxicity-induced dilapidation of chloroplasts and modification in its interior membranes, which adversely affect the photosynthetic pigments and the rate of carbon assimilation. Arsenic negatively affects the Chl a content and Chl b content, maximal photochemical efficiency of PSII (Fv/Fm), the actual PSII photochemical efficiency (ΦPSII), the quantum yield of CO2 assimilation (ΦCO2), and the non-photochemical quenching (NPQ), net photosynthesis rate (A), stomatal conductance to water vapor (gs) and internal CO2 concentration (Ci) in Pistia stratiotes L. plants. The final result of As toxicity was lowered starch concentration, sucrose concentration, and glucose concentration in P. stratiotes [70].
Overall, As toxicity hampers crop growth by altering root plasmolysis, reducing photosynthetic attributes such as degradation of pigments, reduction of the rate of CO2 fixation, reduction of stomatal conductance, and distortion of cell membranes integrity.
4. Arsenic Toxicity and ROS Generation in Plants
ROS generation is a common response in abiotic and biotic stresses [10]. ROS overproduction impaired plant health under stress by adversely affecting range of physiological process including lipid metabolism, DNA, photosynthesis, respiration, enzyme deactivation and growth retardation [71]. Several studies demonstrated As(III) and As(V) induce generation of ROS viz. superoxide (O2•−), the hydroxyl radical (OH•), and H2O2 [72,73]. As(III) is more detrimental to plant growth and generate more O2•− than As(V), which generate more H2O2 [74]. Although root cells sense first As, though generation of ROS started in leaves well before the As accumulation in the leaves tissues, suggested that root cells communicate As toxicity to leaves, probably by H2O2 [75]. Under aerobic condition, As(V) is the main form which enter plant roots by phosphate transporter and within the cell it transform into As(III), which is the main source of ROS generation (Figure 3); [76]. The conversion of As(V) into As(III) is both, enzymatic and nonenzymatic [4]. Enzymatic reaction mediated by arsenate reductase (glutaredoxin) where GSH acts as electron donor [77]. This reduction is followed by methylation process and produces MMA, DMA, tetramethyalarsonium ion (TETRA) and trimethylarsonium oxide (TMAO), arsenocholine, arsenobetaine and arseno-sugars [78]. These methylated products react directly with molecular oxygen and produce ROS. Non enzymatic reduction of As(V) into As(III) occurs through GSH [79]. This conversion, further causes severe oxidative stress as As(III) bind and consume GSH, and impairs antioxidant system. In chloroplast, As(V) is reduced into As(III) by cytochrome/cytochrome oxidase, disturbed electron transport chain and generated ROS [40,70]. In root meristematic cells, mitochondrial arsenate reductase is also found and transforms As(V) into As(III) [80].
Figure 3.
Schematic overview of ROS generation in plant cell under As-stress. Phosphate transporter (PHT) and aquaporins (AQPs) facilitate entry of As(V) and As(III), respectively, into the cell. Initial ROS burst occurs due to arsenate reductase (AsR) mediated and non-enzymatic transformation of As(V) into As(III) in cytoplasm, chloroplast and mitochondria. Subsequently, a second sequential ROS burst occurs due to methylation of As (III) into other organic arsenic metabolites viz. monomethylarsinic acid (MMA), dimethylarsinic acid (DMA), tetraethyalarsonium ion oxide (TETRA), trimethylarsonium oxide (TMAO), arsenobetaine, arsenochlorine and arsenosugars.
Lipid peroxidation, a common toxic effect of As induced ROS, also observed in hyperaccumulating P. vittata [13], hampered cellular and membrane functions [81]. Lipid peroxidation due to ROS is mostly monitored as malondialdehyde (MDA) content, a main product of lipid peroxidation, along with membrane leakage [11,82]. Overproduction of ROS increases polyunsaturated fatty acid (PUFA) and reduces saturated fatty acid of membrane lipids and membrane fluidity, thereby increases membrane leakage [72,83]. ROS also affects enzyme and protein structure and activity by oxidation of side chains, cross-linking and inducing fragmentation of backbone [5,84]. ROS generation under As-stress also modifies nitrogenase base, nucleotide deletion, disrupts protein-DNA binding and may lead DNA cracks [85,86] (Figure 4). In Pisum sativum, chromosome or microtubule damage has been reported under As stress which restricted root meristem activity [87]. Restricted root growth under As-stress may attribute to ROS-induced arrest of mitotic division due to down regulation of cell cycle genes and slow progression of G1 to G2 and from S to M stage, and decreases mitotic index (number of cells progressing into mitosis to the total number of cells) [88,89]. Root growth is also restricted due to root tip death. ROS induces programmed cell death by affecting vacuolar processing enzymes, signaling and triggers programmed cell death [90]. As toxicity caused asymmetric distribution of peroxisomes in A. thaliana root cells and a greater number of peroxisomes occurs in root meristematic zone as compared to root differentiation zone, and the higher peroxisomal ROS generation at root tip induces programmed cell death [91]. The differences in peroxisomal number may be due to As-induced pexophagy, a selective autophagy of peroxisomes [92]. Though it seems roots may have strong antioxidant defense against As toxicity than leaves [46], growing evidence suggested that root gravitropism, cell death, stomatal regulation and other growth and developmental response, under varied abiotic stresses are results of interplay between ROS and phytohormones [93,94]. The ROS and hormonal interplay control gene expression and induce stress responses. As stress upregulated abscisic acid, ethylene and jasmonic acid signaling [95]. ROS generated in chloroplast and mitochondria disrupt ETC by damaging internal and outer membranes of chloroplast and mitochondria [70]. The disruption of chloroplast membrane reduced photosynthetic pigment and carbon fixation [68,96]. Even, chloroplast membrane of old leaves of As hyperaccumulator, P. vittata was also disrupted with high accumulation of As [67].
Figure 4.
Detrimental effects of reactive oxygen species on cellular component and their consequences (rectangle box, outside the cell) under arsenic stress.
5. Arsenic-Induced Oxidative Stress in Plants
Arsenic accumulation in plant tissue generates oxidative stress, mainly during detoxification into less toxic metabolites and disruption of electron transport chain in chloroplast and mitochondria. Oxidative stress was accessed in diverse group of plants (Table 1) under As-stress. Rice, a hyperaccumulating species, also exhibited enhanced H2O2 and thiobarbituric acid reactive substance (TBARS) content when seedlings were subjected to 50 μM As-stress up to 30 days [97]. Arikan et al. [98] also observed similar higher H2O2 and TBARS content in 14-day-old Z. mays seedlings under hydroponic condition with 100 μM As(V). Alsahli et al. [99] observed 69% EL from P. sativum tissues under As-stress (NaAsO2; 20 μM) as compared to only 10% EL from non-stress control condition. Annual and perennial ryegrass when supplied NaAsO2 (2.51 mg mL−1) both exhibited marked increase in O2•− content in mature, expanded and emerging leaves at 60 days, and the content reached up to 65% in emerging leave of annual ryegrass [100]. Similarly, when soybean seedling experienced As stress (NaAsO2, 10 and 100 μM), ROS viz. O2•−, OH• and H2O2 remarkably increased within 5 days and due to this ROS burst, LOX activity also enhanced [5].
Table 1.
Oxidative stress in different plant species under arsenic stress.
6. Antioxidants and Arsenic Tolerance
The plant response to As and other abiotic stresses includes key ROS-scavenging enzymes such as: SOD, CAT, APX, MDHAR, DHAR, GR, GST, GPX, and POD [105,106]. The orchestration of antioxidant defense is performed by the balance of different enzymatic antioxidant, which involve removal of O2•− (SOD), conversion of H2O2 into water and molecular oxygen (CAT), scavenging of H2O2 in the extra-cellular space (POD), conjugation of GSH to electrophilic compounds or hydrophobic compounds (GST), maintenance of ascorbate pool (MDHAR and DHAR), and scavenging of H2O2 to water using ascorbate as specific electron donor (APX) [106].
Several proteomic investigations have observed the differential accumulation of antioxidant enzymes in plant tissues after As exposure (Table 2). Findings regarding this subject are important to gain information on As-induced antioxidant regulation at the translational level. However, more studies are needed on this subject in order to elucidate the relationship between antioxidant enzyme concentration and enzyme activity that is modulated by As exposure in plants. Further research is also needed in order to perform the qualitative evaluation involving isozyme profiling by gel-based approaches, which already performed by some authors that evaluated As-exposed plants [28,107]. Knowledge and achievements regarding As-induced oxidative stress tolerance might also be improved by using emerging proteomic approaches in the field of abiotic stress. For example, phosphoproteomics has been used to unravel plant tolerance mechanisms to heavy metals [108], even though there is a lack of information on this subject related to As toxicity.
Table 2.
Some examples of proteomic studies involving the quantification of antioxidant enzymes in As-exposed plants.
Despite the role that is played by enzymatic antioxidants, a more complete picture of the scavenging capacity in plants upon exposure to As can be achieved by the determination of non-enzymatic antioxidant molecules [41,117,118]. Components of the non-enzymatic antioxidant machinery include GSH, AsA, phenolic compounds (e.g., flavonoids), proline (Pro), cysteine, methionine, carotenoids, α-tocopherol, polyamines, and sugars, as well as emerging components (e.g., anexins and dehydrins) [119]. Also noteworthy, metabolomic approaches have been contributed to in-depth understanding of As-related non-enzymatic antioxidants accumulation [43,120,121].
Many investigations have provided insights into mechanisms underlying antioxidant response of plants to As stress by evaluating changes in antioxidant enzyme activities and non-enzymatic antioxidant contents. Variations between results on this subject is explained to the effects of As, which are dose-, plant species- and experimental conditions-dependent [83,122,123,124,125]. For example, Bianucci et al. [126] observed that SOD, CAT, and GST augmented as well as overall decrease in GR and GPX activities and increased GSH contents under As exposure in a dose-dependent manner. These authors also identified the strong induction of GST activity as suitable biomarker of As toxicity in peanut plants. In another study, the activity of SOD, POX, and GR in Lemna gibba increased while concentration of As increased. In these plants, the anthocyanin content increased constantly, whereas CAT and APX activities as well as the content of chloroplastic pigments were reduced [127]. A higher POD activity in leaves, a reduced POD activity in roots, and induction of SOD and CAT activities in both leaves and roots were caused by As(V) addition in the growth medium of V. faba plants. In rice, the effects of As(III) treatment on the enhanced level of AsA and GSH as well as increased SOD, CAT, APX, chloroplast APX, GPOX, GR, and MDHAR activities were observed [128]. An investigation aimed at evaluating plants of Azolla caroliniana exposed to different concentrations of As found that, unlike the enzymatic molecules, some nonenzymatic antioxidants (e.g., anthocyanin) increased and were positively correlated with As concentration [129].
The existing and potential information derived from studies on As stress response confirms the importance of antioxidants towards helping plants to remove ROS. However, in several plant species, differences between antioxidant related As stress response parameters versus the ones related to As tolerance remain largely unknown. With regards to this focus, the comparative evaluation of As-tolerant and As-sensitive plants (or the comparison of plants with different degrees of tolerance/sensitivity, which includes As-hyperaccumulator plants and their sensitive counterparts) offer huge opportunities for deeper understanding of the contribution of antioxidants to As-induced oxidative stress tolerance. By evaluating two contrasting tobacco genotypes (As-sensitive Nicotiana sylvestris and As-tolerant N. tabacum, cv. ‘Wisconsin’), some authors found meaningful differences in the carbohydrate status. Moreover, a higher total antioxidant capacity based on levels of antioxidant contents (e.g., AsA, GSH, and phenolic compounds) and activities was observed in the As-tolerant genotype [41]. In the study performed by Singh et al. [107], the castor tolerant genotypes presented increased SOD and GPX activities in roots, whereas castor sensitive genotypes showed decreases regarding these enzymes in a As concentration-dependent manner. CAT activity and Pro content were found to be increased in sensitive castor plants and unchanged in tolerant ones due to As(V) treatment [107]. The contents of Pro, GSH, AsA, activities of APX and CAT were used as parameters in observing the higher As sensitivity of O. sativa cv. Khitish compared to cv. Nayanmani [130]. These investigations showed a complex variation in contents or activities according to different factors such as plant genotype, age, organ, as well as the time-length of plant exposure, and As concentration in the growing media. Noteworthy, a better antioxidant performance is not always explained by As-induced increases in non-enzymatic levels or enzyme activities of As-tolerant plants. Instead, there is a complex regulation involving the antioxidant related highest As tolerance degree, which depends on experimental conditions of investigations on this research field and peculiarly regarding the comparison relative to sensitive or less tolerant plants (Table 3).
Table 3.
Examples of studies involving the evaluation of antioxidant molecules in contrasting plants for arsenic tolerance.
7. Approaches in Enhancing Oxidative Stress Tolerance in Plants Exposed to Arsenic
Thirst of plants researchers are increasing for searching and establishing proper strategies to increase plant defense mechanisms upon As-induced oxidative stress. Therefore, exogenous different elicitors like plant nutrients, hormone, antioxidants, osmolytes, signaling molecules, different chelating agents, microbial inoculants, organic amendments etc. were used in different plant species upon exposure to As stress to evaluate their roles in reducing oxidative injury through upregulating antioxidants activities (Table 4).
Table 4.
Exogenous elicitors-mediated oxidative stress tolerance in plant under arsenic toxicity.
7.1. Use of Plant Nutrients
Different plant nutrient receiving attention for their ability to mitigate the oxidative stress and damage upon As exposure [156,157]. Calcium (Ca)-induced lower oxidative stress was reported by Rahman et al. [156] in O. sativa upon As stress, while without stress condition, Ca did not showed any changes in H2O2 and MDA levels. Calcium supplementation increased antioxidants activities including SOD, CAT, GPX, GST in As-stressed rice which contributed in reduction of H2O2 [156]. Calcium also causes the stimulation of AsA-GSH pool in plants upon As toxicity which has strong relationship in regulation of H2O2 detoxification and thus enhances oxidative stress tolerance with lower MDA level. For instance, higher APX, MDHAR, DHAR activities with lower GR activity caused increment of AsA/DHA and GSH/GSSG redox balance along with lower oxidative stress in As-treated rice with Ca [156]. Exogenous application of Ca and sulfur (S) significantly modulating ROS detoxification in As-stressed plant through strengthening the antioxidants responses [157]. Lower H2O2 accumulation by S and Ca in separate and as well as combined application resulted in reduction of MDA in As-stressed Brassica plants where Ca caused comparatively better results [157]. In addition, Ca and S-treated Brassica showed higher AsA/DHA and GSH/GSSG redox in both root and leaves tissue which were because of Ca and S-mediated elevated APX, DHAR and GR activities and thus resulted in lower ROS [157]. Arsenic-induced oxidative stress was mediated by Ca supplementation which caused higher tolerance in V. faba by suppressing both ROS generation and respective enzymatic activity resulted in lower EL and MDA level [73]. This Ca-induced higher As-tolerance was stronger in combination with melatonin where highest reduction of oxidative damage was measured along with elevated activity of antioxidant system including SOD, APX, GR, MDHAR, DHAR and GST activities.
7.2. Use of Phytohormones
Phytohormones are very potential to improve the plant antioxidant defense mechanism consisting of both enzymatic and non-enzymatic stuffs for suppressing metal-induced oxidative damage [158]. Methyl jasmonate (MeJA), for example, is effective to reduce oxidative stress as revealed by lowered ROS generation, elevated redox state of AsA and GSH, strengthened enzymatic antioxidants activities and better membrane stability in plants upon As toxicity [159,160]. Exogenously 1 µM MeJA caused the significant reduction of H2O2 and OH• about 20 and 17%, respectively led to decrease in lipid peroxidation (as MDA; about 27%) in 200 µM As-exposed B. napus [159]. This MeJA-induced oxidative stress tolerance in As-stressed B. napus was acquired due to increasing plant antioxidant defense mechanism through elevated AsA and GSH content along with higher activities of enzymatic components like SOD, POD, CAT, APX and GR. Likely, As-stressed rice showed lower membrane damage revealed by reduced MDA and EL with the application of MeJA led to decrease activities of SOD, POD, CAT and APX [160]. Such MeJA-induced lower membrane damage in As-stressed plants describe the lower generation of ROS which also correlated with the lesser activity of enzymatic antioxidants. Ascorbate-glutathione cycle is one of the vital mechanisms for regulating H2O2 metabolism in plant cell and thus keep its level beyond toxic, which is also strengthened by phytohormones supplementation under As stress [125,144]. The higher AsA-GSH redox status by plant hormones thus contributed in reduction of ROS and consequent oxidative damage like membrane injury, for instance, salicylic acid (SA)-mediated lower H2O2, MDA production and EL in As-stressed Z. mays [144]. Methyl jasmonate diminished oxidative stress through increasing the activity of antioxidant enzymes and decreasing As accumulation by modulating arsenic transporters of rice plants. Addition of MeJA in rice plants under As stress improved the level of AsA, AsA/DHA, GSH and GSH/GSSG, increased the activity SOD, APX and POD. The oxidative stress (H2O2 and MDA) was decreased in those MeJA treated rice plants. The augmented tolerance of those rice plants was also observed in terms of increased Chl content, Chl fluorescence and biomass production, yield components and yield [161].
Similarly, other phytohormones are also significant in reducing As-induced oxidative stress through strengthening antioxidant defense mechanism. For instance, exogenous application of jasmonic acid alleviated the As-induced oxidative stress by 36% of reducing ROS with elevated activity of SOD, CAT, APX and GR in L. valdiviana [74], while cytokinin (e.g., kinetin)-induced lower down of ROS in As-stressed P. cretica [162]. The abscisic acid (10 μM) was used in O. sativa as pretreatment for 24 h to strengthen As tolerance and this pretreatment caused the upto 50 and 38% reduction of O2•− and H2O2, respectively which resulted in 48% lower down of lipid oxidation with improvement of membrane stability [125]. This ABA-mediated relief of oxidative damage in As-stressed plant through ABA-induced elevated response of AsA-GSH pathway. Such As-mediated oxidative stress was downregulated by the exogenous SA in Z. mays [144]. Therefore, exogenous plant hormones are potential candidates for regulating As-induced oxidative stress for increasing plant tolerance through strengthening the plant antioxidant defense mechanism including both non-enzymatic and enzymatic components (Table 4).
7.3. Use of Signaling Molecules
Supplementation of signaling molecules like nitric oxide (NO), hydrogen sulfide (H2S) and H2O2 causes the stimulation in the antioxidants system, leads to reduction of oxidative stress in plants. We summarize the involvement of the signaling behavior of these in suppressing the As-mediated oxidative stress (Table 4).
Exposure of As-induced higher ROS and structural injury of cellular integrity including lipid peroxidation and membrane injury were significantly improved in all NO, H2S and H2O2-treated plants [99,157,163]. The accumulation of ROS was reduced in signaling molecules treated As-stressed plant, for instance, both NO and H2S reduced O2•− and H2O2, OH• accumulation while exogenous application of lower concentration of H2O2 has the capability to suppress O2•− and H2O2 later resulted in better cellular function as well as lowered the oxidative damage as caused lower lipid and protein oxidation. Consequently, regulation of As-induced ROS metabolism requires the intensive involvement of antioxidants activities. Other studies reported about the participation of NO, H2S and H2O2 as external approaches to empower both enzymatic and non-enzymatic antioxidants directly or indirectly to mitigate As-induced oxidative stress [99,145,147].
Exogenous sodium nitroprusside (SNP; as NO donor) in presence of As caused the reduction of enzymatic antioxidants activity like SOD, CAT and POD which in accordance with NO-induced lowered level of O2•−, H2O2, EL by 1.4-, 1.5- and 1.5-fold with lower MDA in Spirodela intermedia [164]. Transcriptional expression of the PCS, GSH1, MT2, and ABC1 were improved by NO supplementation in As stressed tomato plants which increased sequestration of As in root and decreased further translocation of As to the shoot. Exogenous NO also modulated proline metabolism and caused higher accumulation of GSH. The resulted oxidative stress relaxation was evident from H2O2 reduction and protection of photosynthetic apparatus [165]. In another study, the function of nitrate reductase (NR)-synthesized nitric oxide (NO) in the MeJA-induced tolerance of arsenic (As) stress was studied in rice. The positive effects were clear from the increased expression of GSH1, PCS, and ABCC1 genes, higher GSH and PCs contents in the roots and leaves, and increased activity of SOD, CAT, APX and GR. The ultimate oxidative stress reduction is apparent from decreased H2O2, MDA and EL [166]. As an emerging signaling molecule, H2S regulates the key antioxidants activities for keeping lower-level ROS and subsequent better integrity of cellular components. In P. sativum, non-enzymatic antioxidants AsA and GSH contents were elevated with the supplementation of H2S in exposure to As through the higher activity of responsible enzymes like APX, MDHAR, DHAR and GR [99]. Therefore, both of AsA and GSH were actively worked on scavenging As-induced higher H2O2 level through the regulation of the redox status of AsA and GSH. Not only that, exogenous H2S also raised the activity of SOD, and CAT which are also acted on O2•− converting into H2O2 for further action by AsA-GSH cycle. In this study, higher GST activity and GSH also described the roles of GSH in detoxification of lipid and protein peroxidation products used as substrate and thus recovered plant from oxidative status. Although H2O2 is harmful at extreme level but under threshold level it also acts as signaling molecules to regulate plant stress tolerance. Regarding this, it was reported that exogenous H2O2 (1 µM) regulated the ROS metabolism to keep them under beneficial level through the activation of APX, MDHAR, DHAR, and GR in stressed plants due to its signaling roles [157]. However, the actual mechanism of signaling molecules-mediated plants recovery upon As stress is still lacking which demand further extensive studies.
7.4. Use of Chelating Agents
Chelating agents mediated higher upregulation of plant antioxidant defense system for getting relief from As-induced oxidative stress is still not explored widely. Therefore, this approach for getting As-tolerance behavior in cultivated crop species could be vital as these also have metal elimination properties. Citric acid (CA) is known as harmless compound which is able to increase the plant antioxidants capability and thus reduced As-induced oxidative damage through declining the ROS accumulation and lipid peroxidation [167]. Citric acid mediated mitigation of oxidative stress and the plant tolerance in As exposure was due to the upregulation of antioxidant enzymes like SOD, CAT, and [149]. However, the role of chelating compound is very species-dependent along with their dose level. Effect of ethylenediaminetetraacetic acid (EDTA) was studied in regulation of As-induced oxidative stress by declining ROS and lipid peroxidation [168,169]. Application of EDTA enhanced As-induced H2O2 production, but reduced lipid peroxidation [169].
7.5. Use of Soil Amendments
Soil amendments are an eco-friendly and cost-effective approach for betterment of soil health to achieve food safety in this era of climate change. Therefore, researchers have been tried biochar to amend As toxicity and thus improve plant tolerance. Toxic level of As treated higher oxidative stress markers like membrane damage, H2O2 and MDA in G. max were declined when biochar (made from waste wood chips) was applied [170]. Due to the addition of biochar antioxidants defense mechanisms were upregulated in As-treated plants, for instance, SOD, CAT, APX, GPX, GR and GST oxidative injury was prohibited significantly resulted in protection of G. max for oxidative stress [170].
Peanut and canola straw biochar was used to evaluate its potentiality as an organic amendment to improve plant tolerance and growth upon As toxicity [171]. This greenhouse-based study showed the protective effects of biochar on suppressing As-induced oxidative stress (indicated by lowering MDA, H2O2 and O2•− about 82, 49, and 45%, respectively) in soybean which gave the indication of biochar mediated stronger antioxidants defense mechanism in stressed plant and forecast its future useability. Kamran et al. [171] also disclosed about the comparative better performance of peanut straw biochar than canola based.
7.6. Use of Beneficial Microbes
Microbial inoculants effectively regulate the plant antioxidants defense capacity upon As-induced oxidative stress and thus enhance plant tolerance [172]. In addition, this protective effects of microbes in stimulating plant antioxidants mechanism depends on microbes’ species, stains which can be said as strain-specific or specifically antioxidants-specific, As toxicity levels and plants species [173]. Bacterial influence for plant has been documented as beneficial in some extent. Previously, some researchers reported about plant growth-promoting rhizobacteria (PGPR) significantly regulated plant antioxidants enzymes activity. About 100 mg kg−1 of both As(III) and As(V) treatments-induced higher enzymatic antioxidants responses were reduced significantly in V. radiata [174]. Incubation of As-stressed V. radiata with Exiguobacterium showed lower activity of SOD, CAT, APX and GPX near to control treatment thus resulted bacteria-mediated suppression of oxidative stress (as lessening ROS generation. Likely, several PGPR documented for increasing antioxidants activity like SOD by Bacillus cereus [175], SOD and CAT by Populus deltoides [176], APX and CAT by B. licheniformis [177], SOD and CAT (about 27 and 62%, respectively) by B. aryabhattai [178] in As-stressed plant. Consequently, in recent study of Xiao et al. [172] was about modulation of antioxidants defense system in As-stressed rice by different PGPR for attuning lower ROS production. Pseudomonas mosselii, B. thuringiensis, and Bacillus sp. JBS-28 inoculation showed the reduction of As-mediated oxidative damage through promoting the antioxidants capacity like SOD and POX activity which directly scavenge the ROS. Thereafter, in case of wheat, Brevundimonas intermedia and P. gessardii modulated higher SOD and APX activities were revealed by the higher expression of their respective gene at As exposure [179]. Ghosh et al. [180] reported about Pantoea dispersa–modulated higher SOD and CAT activities with less MDA and thus As-tolerant bacterial strains were recommended for using in improving membrane stability of O. sativa upon As toxicity. However, the innate mechanisms in antioxidant defense modulation in As-stressed plants by PGPR are still unknown and which demand further extensive studies. Piriformospora indica improved the root sequestration of As, decreased As translocation and improved the AsA-GSH homeostasis which altogether contributed better photosynthetic performance and reduced the oxidative stress. P. indica sequestrated As in the roots through upregulating the expression of PCS1 and PCS2 genes. It also reduced As accumulation in shoot by downregulating the expression of Lsi2, Lsi6, Nramp1 and Nramp5. Modulating AsA-GSH homeostasis P. indica decreased the MDA level of rice plant [181].
7.7. Other Chemical Elicitors
Plant researchers are also interested to explore the new, most adaptive and efficient technology for increasing plant tolerance against As stress. Therefore, antioxidants, osmolytes, polyamine and other chemical elicitors likely have been used in small scale previously and still now need more exploration to understand and develop these exogenous protectant-mediated mechanisms involved in plant oxidative stress tolerance. Notable, melatonin has gained the attention of plant researchers’ community due to its antioxidant’s potentiality specially its mitigating nature against the oxidative stress-mediated cellular damage [182]. Exogenous melatonin caused the stimulation in defense system of rosemary seedlings upon As stress as it improved cell membrane integrity with reduction of oxidative damage through increment of enzymatic antioxidants capacity [183]. Samanta et al. [184] reported that melatonin treatment improved As-induced oxidative stress tolerance by triggering the antioxidative machinery where increased the total antioxidants activity with elevated non-enzymatic antioxidants content like AsA, phenolic compound resulted in the reduction of oxidative damage. Similarly, melatonin-mediated reduction of ROS with upregulation of antioxidants activity like APX, SOD, CAT, POD was reported in As-stressed Camellia sinensis [153].
As stress management approach, use of non-enzymatic antioxidants is also efficient for suppressing oxidative stress by improving plant antioxidant capacity of plant upon As-toxicity. Exogenous AsA (250 and 500 mg kg−1) showed the amelioration of 15 µM As-induced oxidative stress through enhancing the capacity of AsA-GSH cycle in rice maintaining the sufficient level of both AsA and GSH [185]. Ascorbate-treated plant showed the reduction of ROS and MDA contents as indication of lowered oxidative damage with higher AsA/DHA and GSH/GSSG ratios. Jung et al. [186] studied the role of exogenous GSH (50 and 100 mg kg−1) on biochemical responses of ROS and antioxidant levels in 14 d-old O. sativa seedlings at As (15 µM) exposure. This GSH treatment reversed the As-induced oxidative damage with the improvement of antioxidants activity. Hydroponically grown rice seedling with the foliar application of GSH declined As-induced oxidative stress indicated by lower ROS (O2•− and H2O2) and lipid peroxidation (MDA content), whereas increased the redox balance of AsA/DHA and GSH/GSSG with higher activity of MDHAR, DHAR and GR. Therefore, it can be suggested from both of above-mentioned studies that exogenous AsA and GSH causes the higher induction of AsA–GSH cycle, which re-established the cellular redox status.
The osmolyte Pro also regulates antioxidants capacity in stressed plant besides of its role on maintaining osmotic status. As a vital amino acid, Pro helps in scavenging stress-mediated higher ROS and protects plants from oxidative damage and thus stabilizes cellular structure including membrane [163]. In the experiment [163], Pro (25 μM) was applied in As-treated (25 μM) Solanum melongena and Pro fed plants showed the decline of O2•−, H2O2 and MDA level which were elevated in stress treatment alone which were because of the stimulation in activities of SOD, CAT and POD.
Phenolic compounds like chlorogenic acid and hesperidin are also well recognized as non-enzymatic antioxidants those are strongly able to neutralize the harmful free radicals besides of their metal chelating actions. Both chlorogenic (100 μM) and hesperidin (50 μM) were selected for using them singly or combined on maize plants upon As-stress (100 μM) [98]. This treatment altered the stress-induced reduction of antioxidants mechanism in maize by elevated the actions of SOD, CAT, POD, GST, GPX, MDHAR and GR which resulted in suppressing of ROS and TBARS content with maintaining higher redox status of AsA/DHA and GSH/GSSG. Thus, phenolic compounds are able to contributing in maintaining the cellular redox balance through the regulating the AsA-GSH cycle along with other potential antioxidants enzymes activities [98].
In recent years, nanoparticles (NPs), which are ultrafine particles presenting at least one dimension in <100 nm range, have gained much attention in topics related to modern agricultural research [187]. This novel and emerging nanotechnology approach has been reported to improve the production of some plant species by enhancing tolerance to environmental stresses [187,188] and promote beneficial changes regarding antioxidants. This includes increased enzyme activities and non-enzymatic contents in As-exposed plants of several species such as rice [189,190,191], soybean [192], maize [193], tomato [194] and mung bean [195]. Thus, besides covering the field of environmental protection and As toxicity alleviation in plants [196,197], the potential application of NPs highlights the role of antioxidant enzymes and non-enzymatic antioxidant molecules as important molecules for the modulation of tolerance to As-induced oxidative stress. Zinc nanoparticles (ZNO NPs) positively affect As-induced oxidative stress in rice by stimulating enzymatic antioxidants activity including SOD and CAT which lead to about 13–30% reduction of MDA content [198]. Similarly, ZNO NPs mediated further higher SOD activity was also measured in As-stressed (2 mg L−1) rice where 10 and 100 mg L−1 concentration of ZnO NP showed better results [190].
8. Genetic Engineering in Enhancing Antioxidant Defense towards Arsenic Tolerance
Under increasing As concentrations, plants suffer a redox imbalance resulting in an increase in ROS levels which induces damages on the cellular biomolecules and functions [199]. Beside to the current techniques used for reduction of As in soil and water remediation, transgenic approaches have to be strengthened to solve this problem [200]. These approaches can be addressed considering different criteria such as working with genes responsible for As absorption, movement and sequestration in vacuoles, and enzymes and proteins regulating As conversion and GSH and PC metabolism [201].
Regarding As transporters, they can be classified as plasma membrane or vacuole transporters. The main plasma membrane transporters are aquaglyceroporins and phosphate transporters (PHTs) involved in the uptake process of the inorganic forms of As(III and V) [202]. Belonging to the group of aquaglyceroporins are NIPs (Nodulin 26-like Intrinsic Proteins) which participate in a selective import of As(III) and not As(V) to the xylem vessels from the external medium [22,27]. In the case of phosphate transporters, the similarity between As(V) and phosphate and their affinity for phosphate transporters led to genetic approaches based on the knockdown or knockout of the genes involved in phosphate transporters to develop As tolerant crops [19]. Vacuole transporters are also of crucial interest in the establishment of As tolerant crop varieties, since they are involved in the restriction of As movement in a plant through the complexation of As(III) with PC into storage organelles like vacuoles. ATP binding cassette (ABC) transporter family members such as ABCC1 and ABCC2 are included in this group of As transporters [29].
Arsenate reductase are enzymes involved in the conversion of As (V) to As (III) in plants and the overexpression of the genes involved in this enzymatic activities are particularly relevant to improve the As tolerance of crops. Some of these genes are arsenate tolerance QTL1 (ATQ1) [203], and high As content 1 (HAC1) and HAC4 [204,205].
Genetic engineering approaches with glutaredoxins are also required to regulate the redox status of the cells against As toxicity [206]. These cysteine rich proteins are able to reduce the disulphides through reduced GSH [72].
The detoxification of As toxicity in plants is carried out through sequestration with GSH and phytochelatins due to the high affinity of sulfhydryl (-SH) groups of these compounds with As or vacuolar sequestration [22,207]. Glutathione S-transferases are responsible of the reduction of oxidative damage in cells conjugating reactive molecules with GSH [208]. These enzymes through the conjugation process of thiol group of GSH with electrophile substrates can reduces the toxicity in cells sequestering these reactive substrates in vacuoles or being effluxed from cells through ATP dependent pumps [209]. Phytochelatins are vacuolar transporters involved in the sequestration of metalloids such as As into the vacuole, therefore, the establishment of transgenics crops with upregulated genes expression involved in metal resistance are of special interest [210]. It is necessary to point out that the biosynthesis of phytochelatins and GST are dependent on sulphate uptake and conversion to cysteine [211].
Beside to the above-mentioned key genes involved in As tolerance, transcription factors are also considered crucial in the tolerance against this metalloid. Several examples include Zinc-Finger type [212]; bZIP [30]; GeBP-LIKE 4 (GPL4) [213]; NAC [214]; R2R3-type MYB [215]. Moreover, kinases responsible for the regulation of the transcription process like mitogen activated protein (MAP) kinase, SNF1-related kinases (SnRKs) and leucine-rich repeat receptor-like kinase VIII (LRR-RLK VIII) are strengthened in genetic engineering approaches in crops with higher tolerance to As [199].
Several examples about genetic engineering strategies above mentioned carried out in different species to improve the tolerance to As are included in Table 5.
Table 5.
Genetic engineering approaches for As tolerance and redox and metabolite changes.
9. Conclusions
Arsenic toxicity is a serious issue as it is not only being uptaken by human through drinking water but also uptaken through plants and animals through the food chain. The productivity of plants is also hampering due to As toxicity. There are hundreds of unanswered questions in the mechanism of As uptake, efflux, translocation, accumulation and detoxification in plants. Only few membrane proteins/transporters have identified in very few plant species. Some research findings proved that As use same transporters [e.g., aquaporins, AQPs: OsNIP (Lsi1, Lsi2; phosphate transporter, OsPHT] with some other elements. There might be other transporters which should be identified through intrinsic research. Those research findings can be vital for selecting exogenous phytoprotectants/fertilizers which may reduce As uptake by root and then translocation to the following parts of the plants. Mechanism of transportation of As through vascular tissue is not explored completely. The mechanisms and pathways how the As cause oxidative stress that should be focused in diverse way. Plants with enhanced antioxidant defense system under As stress should be recognized and those should be incorporated in various plant improvement programs. Finding out microorganisms and allelochemicals releasing plants which can bind and reduce the As uptake of desired crop can be taken under consideration. Identifying the As hyperaccumulation plants from nature is necessary. Very little is known about the mechanism of As transport and accumulation in different crops/plants including the As hyperaccumulator and non-hyperaccumulator. Then, it will possible to cleanup As contaminated soil, to develop As tolerant plants through breeding, biotechnological or transgenic approaches which will prevent As-induced crop productivity loss and will ensure safe food production for animal or human being. Proteomics, genomics, micromics, transcriptomics, metabolomics, inomics, metallomics approaches can be useful tools for thoughtful realization of the mechanisms of plant response and tolerance to As stress.
Author Contributions
Conceptualization, K.N. and M.H.; writing—original draft preparation, K.N., M.S.R., K.P., K.B., D.N.M., P.G.-C. and M.H.; writing—review and editing, M.H.; visualization, K.N., K.B. and M.H. All authors have read and agreed to the published version of the manuscript.
Funding
This research received no external funding.
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
Not applicable.
Acknowledgments
The authors acknowledge Ayesha Siddika, Salma Binte Salam, Taufika Islam Anee and Shamima Sultana for their help during the organization of the literature and necessary formatting.
Conflicts of Interest
Mirza Hasanuzzaman, who is the coauthor of this article, is a current Editorial Board member of Plants. This fact did not affect the peer-review process. All other authors declare no conflict of interest.
References
- Hasanuzzaman, M.; Nahar, K.; Fujita, M. Arsenic toxicity in plants and possible remediation. In Soil Remediation and Plants: Prospects and Challenges; Hakeem, K.R., Sabir, M., Öztürk, M., Mermut, A.R., Eds.; Academic Press: Amsterdam, The Netherlands, 2015; pp. 433–501. [Google Scholar]
- Chandrakar, V.; Pandey, N.; Keshavkant, S. Plant responses to arsenic toxicity: Morphology and physiology. In Mechanisms of Arsenic Toxicity and Tolerance in Plant; Hasanuzzaman, M., Nahar, K., Fujita, M., Eds.; Springer: Singapore, 2018; pp. 27–48. [Google Scholar]
- Polya, D.A.; Sparrenborn, C.; Datta, S.; Guo, H. Groundwater arsenic biogeochemistry: Key questions and use of tracers to understand arsenic-prone groundwater systems. Geosci. Front. 2019, 10, 1635–1641. [Google Scholar] [CrossRef] [Scilit]
- Finnegan, P.; Chen, W. Arsenic toxicity: The effects on plant metabolism. Front. Physiol. 2012, 3, 182. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chandrakar, V.; Naithani, S.C.; Keshavkant, S. Arsenic-induced metabolic disturbances and their mitigation mechanisms in crop plants: A review. Biologia 2016, 71, 367–377. [Google Scholar] [CrossRef] [Scilit]
- Kumar, V.; Vogelsang, L.; Schmidt, R.R.; Sharma, S.S.; Seidel, T.; Dietz, K.J. Remodeling of root growth under combined arsenic and hypoxia stress is linked to nutrient deprivation. Front. Plant Sci. 2020, 11, 569687. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Garg, N.; Singla, P. Arsenic toxicity in crop plants: Physiological effects and tolerance mechanisms. Environ. Chem. Lett. 2011, 9, 303–321. [Google Scholar] [CrossRef] [Scilit]
- Pandey, C.; Augustine, R.; Panthri, M.; Zia, I.; Bisht, N.C.; Gupta, M. Arsenic affects the production of glucosinolate, thiol and phytochemical compounds: A comparison of two Brassica cultivars. Plant Physiol. Biochem. 2017, 111, 144–154. [Google Scholar] [CrossRef] [Scilit]
- Ali, M.A.; Fahad, S.; Haider, I.; Ahmed, N.; Ahmad, S.; Hussain, S.; Arshad, M. Oxidative stress and antioxidant defense in plants exposed to metal/metalloid toxicity. In Reactive Oxygen, Nitrogen and Sulfur Species in Plants: Production, Metabolism, Signaling and Defense Mechanisms; Hasanuzzaman, M., Fotopoulos, V., Nahar, K., Fujita, M., Eds.; Wiley: Hoboken, NJ, USA, 2019; Volume 1, pp. 353–370. [Google Scholar]
- Hasanuzzaman, M.; Bhuyan, M.H.M.B.; Zulfiqar, F.; Raza, A.; Mohsin, S.M.; Mahmud, J.A.; Fujita, M.; Fotopoulos, V. Reactive oxygen species and antioxidant defense in plants under abiotic stress: Revisiting the crucial role of a universal defense regulator. Antioxidants 2020, 9, 681. [Google Scholar] [CrossRef] [Scilit]
- Gupta, D.K.; Inouhe, M.; Rodríguez-Serrano, M.; Romero-Puerta, M.C.; Sandalio, L.M. Oxidative stress and arsenic toxicity: Role of NADPH oxidases. Chemosphere 2013, 90, 1987–1996. [Google Scholar] [CrossRef] [Scilit]
- Most, P.; Papenbrock, J. Possible roles of plant sulfurtransferases in detoxification of cyanide, reactive oxygen species, selected heavy metals and arsenate. Molecules 2015, 20, 1410–1423. [Google Scholar] [CrossRef] [Scilit]
- Singh, N.; Ma, L.Q.; Srivastava, M.; Rathinasabapathi, B. Metabolic adaptations to arsenic-induced oxidative stress in Pteris vittata L. and Pteris ensiformis L. Plant Sci. 2006, 170, 274–282. [Google Scholar] [CrossRef] [Scilit]
- Khatun, M.; Matsushima, D.; Rhaman, M.S.; Okuma, E.; Nakamura, T.; Nakamura, Y.; Munemasa, S.; Murata, Y. Exogenous proline enhances antioxidant enzyme activities but does not mitigate growth inhibition by selenate stress in tobacco BY-2 cells. Biosci. Biotechnol. Biochem. 2020, 84, 2281–2292. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kaur, N.; Kaur, J.; Grewal, S.K.; Singh, I. Effect of heat stress on antioxidative defense system and its amelioration by heat acclimation and salicylic acid pre-treatments in three pigeonpea genotypes. Indian J. Agric. Biochem. 2019, 32, 106–110. [Google Scholar] [CrossRef] [Scilit]
- Hasanuzzaman, M.; Bhuyan, M.H.M.; Anee, T.I.; Parvin, K.; Nahar, K.; Mahmud, J.A.; Fujita, M. Regulation of ascorbate-glutathione pathway in mitigating oxidative damage in plants under abiotic stress. Antioxidants 2019, 8, 384. [Google Scholar] [CrossRef] [Scilit]
- Kalita, J.; Pradhan, A.K.; Shandilya, Z.M.; Tanti, B. Arsenic stress responses and tolerance in rice: Physiological, cellular and molecular approaches. Rice Sci. 2018, 25, 235–249. [Google Scholar] [CrossRef] [Scilit]
- Shahid, M.; Khalid, S.; Bibi, I.; Khalid, S.; Masood, N.; Qaisrani, S.A.; Niazi, N.K.; Dumat, C. Arsenic-induced oxidative stress in Brassica oleracea: Multivariate and literature data analyses of physiological parameters, applied levels and plant organ type. Environ. Geochem. Health 2021, 1–13. [Google Scholar] [CrossRef] [Scilit]
- Abedi, T.; Mojiri, A. Arsenic uptake and accumulation mechanisms in rice species. Plants 2020, 9, 129. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wolterbeek, H.T.; van der Meer, A.J.G.M. Transport rate of arsenic, cadmium, copper and zinc in Potamogeton pectinatus L.: Radiotracer experiments with 76As, 109,115Cd, 64Cu and 65,69mZn. Sci. Total Environ. 2002, 287, 13–30. [Google Scholar] [CrossRef] [Scilit]
- Kumarathilaka, P.; Seneweera, S.; Meharg, A.; Bundschuh, J. Arsenic accumulation in rice (Oryza sativa L.) is influenced by environment and genetic factors. Sci. Total Environ. 2018, 642, 485–496. [Google Scholar] [CrossRef] [Scilit]
- Zhao, F.J.; Ago, Y.; Mitani, N.; Li, R.Y.; Su, Y.H.; Yamaji, N.; McGrath, S.P.; Ma, J.F. The role of the rice aquaporin Lsi1 in arsenite efflux from roots. New Phytol. 2010, 186, 392–399. [Google Scholar] [CrossRef] [Scilit]
- Sun, H.; Duan, Y.; Qi, X.; Zhang, L.; Huo, H.; Haijun Gong, H. Isolation and functional characterization of CsLsi2, a cucumber silicon efflux transporter gene. Ann. Bot. 2018, 122, 641–648. [Google Scholar] [CrossRef] [Scilit]
- He, Z.; Yan, H.; Chen, Y.; Shen, H.; Xu, W.; Zhang, H.; Shi, L.; Zhu, Y.G.; Ma, M. An aquaporin PvTIP4;1 from Pteris vittata may mediate arsenite uptake. New Phytol. 2016, 209, 746–761. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kamiya, T.; Fujiwara, T. Arabidopsis NIP1;1 transports antimonite and determines antimonite sensitivity. Plant Cell Physiol. 2009, 50, 1977–1981. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xu, W.; Dai, W.; Yan, H.; Li, S.; Shen, H.; Chen, Y.; Xu, H.; Sun, Y.; He, Z.; Ma, M. Arabidopsis NIP3;1 plays an important role in arsenic uptake and root-to-shoot translocation under arsenite stress conditions. Mol. Plant 2015, 8, 722–733. [Google Scholar] [CrossRef] [Scilit]
- Mosa, K.A.; Kumar, K.; Chhikara, S.; Mcdermott, J.; Liu, Z.; Musante, C.; White, J.C.; Dhankher, O.P. Members of rice plasma membrane intrinsic proteins subfamily are involved in arsenite permeability and tolerance in plants. Transgenic Res. 2012, 21, 1265–1277. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Shri, M.; Singh, P.K.; Kidiwai, M.; Gautam, N.; Dubey, S.; Verma, G.; Chakrabarty, D. Recent advances in arsenic metabolism in plants: Current status, challenges and highlighted biotechnological intervention to reduce grain arsenic in rice. Metallomics 2019, 11, 519–532. [Google Scholar] [CrossRef] [Scilit]
- Song, W.Y.; Park, J.; Mendoza-Cózatl, D.G.; Suter-Grotemeyer, M.; Shim, D.; Hörtensteiner, S.; Geisler, M.; Weder, B.; Rea, P.A.; Rentsch, D. Arsenic tolerance in Arabidopsis is mediated by two ABCC-type phytochelatin transporters. Proc. Natl. Acad. Sci. USA 2010, 107, 21187–21192. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, P.; Zhang, W.; Mao, C.; Xu, G.; Zhao, F.J. The role of OsPT8 in arsenate uptake and varietal difference in arsenate tolerance in rice. Environ. Exp. Bot. 2016, 67, 6051–6059. [Google Scholar] [CrossRef] [Scilit]
- Shi, S.; Wang, T.; Chen, Z.; Tang, Z.; Wu, Z.; Salt, D.E.; Chao, D.Y.; Zhao, F.J. OsHAC1; 1 and OsHAC1; 2 function as arsenate reductases and regulate arsenic accumulation. Plant Physiol. 2016, 172, 1708–1719. [Google Scholar] [CrossRef] [Scilit]
- Li, R.Y.; Ago, Y.; Liu, W.J.; Mitani, N.; Feldmann, J.; McGrath, S.P.; Ma, J.F.; Zhao, F.-J. The rice aquaporin Lsi1 mediates uptake of methylated arsenic species. Plant Physiol. 2009, 150, 2071–2080. [Google Scholar] [CrossRef] [Scilit]
- Mishra, S.; Mattusch, J.; Wennrich, R. Accumulation and transformation of inorganic and organic arsenic in rice and role of thiol-complexation to restrict their translocation to shoot. Sci. Rep. 2017, 7, 40522. [Google Scholar] [CrossRef] [Scilit]
- Ye, Y.; Li, P.; Xu, T.; Zeng, L.; Cheng, D.; Yang, M.; Luo, J.; Lian, X. OsPT4 contributes to arsenate uptake and transport in rice. Front. Plant Sci. 2017, 8, 2197. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lin, Y.; Sun, Z.; Li, Z.; Xue, R.; Cui, W.; Sun, S.; Liu, T.; Zeng, R.; Song, Y. Deficiency in silicon transporter Lsi1 compromises inducibility of anti-herbivore defense in rice plants. Front. Plant Sci. 2019, 10, 652. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cao, Y.; Sun, D.; Mei, H.; Liu, X.; Sun, S.; Xu, G.; Liu, Y.; Chen, Y. Knocking out OsPT4 gene decreases arsenate uptake by rice plants and inorganic arsenic accumulation in rice grains. Environ. Sci. Technol. 2017, 51, 12131–12138. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Carey, A.-M.; Scheckel, K.G.; Lombi, E.; Newville, M.; Choi, Y.; Norton, G.J.; Charnock, J.M.; Feldmann, J.; Price, A.H.; Meharg, A.A. Grain unloading of arsenic species in rice. Plant Physiol. 2010, 152, 309–319. [Google Scholar] [CrossRef] [Scilit]
- Mitra, A.; Chatterjee, S.; Moogouei, R.; Gupta, D.K. Arsenic accumulation in rice and probable mitigation approaches: A review. Agronomy 2017, 7, 67. [Google Scholar] [CrossRef] [Scilit]
- Tang, Z.; Chen, Y.; Chen, F.; Ji, Y.; Zhao, F.J. OsPTR7 (OsNPF8.1), a putative peptide transporter in rice, is involved in dimethylarsenate accumulation in rice grain. Plant Cell Physiol. 2017, 58, 904–913. [Google Scholar] [CrossRef] [Scilit]
- Abbas, G.; Murtaza, B.; Bibi, I.; Shahid, M.; Niazi, N.K.; Khan, M.I.; Amjad, M.; Hussain, M. Arsenic uptake, toxicity, detoxification, and speciation in plants: Physiological, biochemical, and molecular aspects. Int. J. Environ. Res. Public Health 2018, 15, 10059. [Google Scholar] [CrossRef] [Scilit]
- Kofroňová, M.; Hrdinová, A.; Mašková, P.; Tremlová, J.; Soudek, P.; Petrová, Š.; Pinkas, D.; Lipavská, H. Multi-component antioxidative system and robust carbohydrate status, the essence of plant arsenic tolerance. Antioxidants 2020, 9, 283. [Google Scholar] [CrossRef] [Scilit]
- Zemanová, V.; Pavlíková, D.; Hnilička, F.; Pavlík, M. Arsenic toxicity-induced physiological and metabolic changes in the shoots of Pteris cretica and Spinacia oleracea. Plants 2021, 10, 2009. [Google Scholar] [CrossRef] [Scilit]
- Martínez-Castillo, J.I.; Saldaña-Roblesa, A.; Ozuna, C. Arsenic stress in plants: A metabolomic perspective. Plant Stress 2022, 3, 100055. [Google Scholar] [CrossRef] [Scilit]
- Patel, H.V.; Parmar, S.R.; Chudasama, C.J.; Mangrola, A.V. Interactive studies of zinc with cadmium and arsenic on seed germination and antioxidant properties of Phaseolus aureus Roxb. Int. J. Plant Anim. Environ. Sci. 2013, 3, 166–174. [Google Scholar]
- Singh, R.; Jha, A.B.; Misra, A.N.; Sharma, P. Differential responses of growth, photosynthesis, oxidative stress, metals accumulation and NRAMP genes in contrasting Ricinus communis genotypes under arsenic stress. Environ. Sci. Pollut. Res. 2019, 26, 31166–31177. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Rodríguez-Ruiz, M.; Aparicio-Chacón, M.V.; Palma, J.M.; Corpas, F.J. Arsenate disrupts ion balance, sulfur and nitric oxide metabolisms in roots and leaves of pea (Pisum sativum L.) plants. Environ. Exp. Bot. 2019, 161, 143–156. [Google Scholar] [CrossRef] [Scilit]
- Nath, S.; Panda, P.; Mishra, S.; Dey, M.; Choudhury, S.; Sahoo, L.; Panda, S.K. Arsenic stress in rice: Redox consequences and regulation by iron. Plant Physiol. Biochem. 2014, 80, 203–210. [Google Scholar] [CrossRef] [Scilit]
- Niazi, N.K.; Bibi, I.; Fatimah, A.; Shahid, M.; Javed, M.T.; Wang, H.; Ok, Y.S.; Bashir, S.; Murtaza, B.; Saqib, Z.A. Phosphate-assisted phytoremediation of arsenic by Brassica napus and Brassica juncea: Morphological and physiological response. Int. J. Phytoremediat. 2017, 19, 670–678. [Google Scholar] [CrossRef] [Scilit]
- Farooq, M.A.; Li, L.; Ali, B.; Gill, R.A.; Ali, B.; Wang, J.; Islam, F.; Ali, S.; Gill, M.B.; Zhou, W. Oxidative injury and antioxidant enzymes regulation in arsenic-exposed seedlings of four Brassica napus L. cultivars. Environ. Sci. Pollut. Res. 2015, 22, 10699–10712. [Google Scholar] [CrossRef] [Scilit]
- Mubarak, H.; Mirza, N.; Chai, L.-Y.; Yang, Z.-H.; Yong, W.; Tang, C.-J.; Mahmood, Q.; Pervez, A.; Farooq, U.; Fahad, S. Biochemical and metabolic changes in arsenic contaminated Boehmeria nivea L. BioMed Res. Int. 2016, 2016, 1423828. [Google Scholar] [CrossRef] [Scilit]
- Garg, N.; Singla, P. The role of Glomus mosseae on key physiological and biochemical parameters of pea plants grown in arsenic contaminated soil. Sci. Hortic. 2012, 143, 92–101. [Google Scholar] [CrossRef] [Scilit]
- Hasanuzzaman, M.; Fujita, M. Exogenous sodium nitroprusside alleviates arsenic-induced oxidative stress in wheat (Triticum aestivum L.) seedlings by enhancing antioxidant defense and glyoxalase system. Ecotoxicology 2013, 22, 584–596. [Google Scholar] [CrossRef] [Scilit]
- Gusman, G.S.; Oliveira, J.A.; Farnese, F.S.; Cambraia, J. Arsenate and arsenite: The toxic effects on photosynthesis and growth of lettuce plants. Acta Physiol. Plant. 2013, 35, 1201–1209. [Google Scholar] [CrossRef] [Scilit]
- Srivastava, S.; Sharma, Y.K. Impact of arsenic toxicity on black gram and its amelioration using phosphate. Int. Sch. Res. Not. 2013, 2013, 340925. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Iriel, A.; Dundas, G.; Cirelli, A.F.; Lagorio, M.G. Effect of arsenic on reflectance spectra and chlorophyll fluorescence of aquatic plants. Chemosphere 2015, 119, 697–703. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Duman, F.; Ozturk, F.; Aydin, Z. Biological responses of duckweed (Lemna minor L.) exposed to the inorganic arsenic species As(III) and As(V): Effects of concentration and duration of exposure. Ecotoxicology 2010, 19, 983–993. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Suneja, Y. Physio-Biochemical Responses and Allelic Diversity for Water Deficit Tolerance Related Traits in Aegilops tauschii and Triticum dicoccoides. Ph.D. Thesis, Punjab Agricultural University, Ludhiana, India, 2014. [Google Scholar]
- Emamverdian, A.; Ding, Y.; Mokhberdoran, F.; Xie, Y. Heavy metal stress and some mechanisms of plant defense response. Sci. World J. 2015, 2015, 756120. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nabi, A.; Naeem, M.; Aftab, T.; Masroor, M.; Khan, A. Arsenic toxicity induced changes in growth, photosynthetic pigments, antioxidant machinery, essential oil, menthol and other active constituents of menthol mint (Mentha arvensis L.). J. Essent. Oil Bear. Plants 2019, 22, 1333–1348. [Google Scholar] [CrossRef] [Scilit]
- Bhattacharya, S.; De Sarkar, N.; Banerjee, P.; Banerjee, S.; Mukherjee, S.; Chattopadhyay, D.; Mukhopadhyay, A. Effects of arsenic toxicity on germination, seedling growth and peroxidase activity in Cicer arietinum. Int. J. Agric. Food Sci. 2012, 2, 131–137. [Google Scholar]
- Fatima, A.; Kataria, S.; Prajapati, R.; Jain, M.; Agrawal, A.K.; Singh, B.; Kashyap, Y.; Tripathi, D.K.; Singh, V.P.; Gadre, R. Magneto-priming effects on arsenic stress-induced morphological and physiological variations in soybean involving synchrotron imaging. Physiol. Plant. 2021, 173, 88–99. [Google Scholar]
- Farooq, M.A.; Islam, F.; Ali, B.; Najeeb, U.; Mao, B.; Gill, R.A.; Yan, G.; Siddique, K.H.M.; Zhou, W. Arsenic toxicity in plants: Cellular and molecular mechanisms of its transport and metabolism. Environ. Exp. Bot. 2016, 132, 42–52. [Google Scholar] [CrossRef] [Scilit]
- Gupta, P.; Bhatnagar, A.K. Spatial distribution of arsenic in different leaf tissues and its effect on structure and development of stomata and trichomes in mung bean, Vigna radiata (L.) Wilczek. Environ. Exp. Bot. 2015, 109, 12–22. [Google Scholar] [CrossRef] [Scilit]
- Armendariz, A.L.; Talano, M.A.; Villasuso, A.L.; Travaglia, C.; Racagni, G.E.; Reinoso, H.; Agostini, E. Arsenic stress induces changes in lipid signaling and evokes the stomata closure in soybean. Plant Physiol. Biochem. 2016, 103, 45–52. [Google Scholar] [CrossRef] [Scilit]
- De Oliveira, A.B.; Alencar, N.L.M.; Gomes-Filho, E. Comparison between the water and salt stress effects on plant growth and development. In Responses of Organisms to Water Stress; Akıncı, S., Ed.; Intech: London, UK, 2013. [Google Scholar] [CrossRef] [Scilit]
- Vezza, M.E.; Llanes, A.; Travaglia, C.; Agostini, E.; Talano, M.A. Arsenic stress effects on root water absorption in soybean plants: Physiological and morphological aspects. Plant Physiol. Biochem. 2018, 123, 8–17. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, W.X.; Chen, T.B.; Huang, Z.C.; Lei, M.; Liao, X.Y. Effect of arsenic on chloroplast ultrastructure and calcium distribution in arsenic hyperaccumulator Pteris vittata L. Chemosphere 2006, 62, 803–809. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Schneider, J.; Labory, C.R.; Rangel, W.M.; Alves, E.; Guilherme, L.R. Anatomy and ultrastructure alterations of Leucaena leucocephala (Lam.) inoculated with mycorrhizal fungi in response to arsenic-contaminated soil. J. Hazard. Mater. 2013, 262, 1245–1258. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Upadhyaya, H.; Shome, S.; Roy, D.; Bhattacharya, M.K. Arsenic induced changes in growth and physiological responses in Vigna radiata seedling: Effect of curcumin interaction. Am. J. Plant Sci. 2014, 5, 3609–3618. [Google Scholar] [CrossRef]
- Farnese, F.S.; Oliveira, J.A.; Paiva, E.A.S.; Menezes-Silva, P.E.; da Silva, A.A.; Campos, F.V.; Ribeiro, C. The Involvement of nitric oxide in Integration of plant physiological and ultrastructural adjustments in response to arsenic. Front. Plant Sci. 2017, 8, 516. [Google Scholar] [CrossRef] [Scilit]
- García-Caparrós, P.; De Filippis, L.; Gul, A.; Hasanuzzaman, M.; Ozturk, M.; Altay, V.; Lao, M.T. Oxidative stress and antioxidant metabolism under adverse environmental conditions: A review. Bot. Rev. 2021, 87, 421–466. [Google Scholar] [CrossRef] [Scilit]
- Mishra, S.; Dwivedi, S.; Mallick, S.; Tripathi, R.D. Redox homeostasis in plants under arsenic stress. In Redox Homeostasis in Plants: From Signalling to Stress Tolerance; Panda, S.K., Yamamoto, Y.Y., Eds.; Springer: Singapore, 2019; pp. 179–198. [Google Scholar]
- Siddiqui, M.H.; Alamri, S.; Khan, M.N.; Corpas, F.J.; Al-Amri, A.A.; Alsubaie, Q.D.; Ali, H.M.; Kalaji, H.M.; Ahmad, P. Melatonin and calcium function synergistically to promote the resilience through ROS metabolism under arsenic-induced stress. J. Hazard. Mater. 2020, 398, 122882. [Google Scholar] [CrossRef] [Scilit]
- Coelho, D.G.; de Andrade, H.M.; Marinato, C.S.; Araujo, S.C.; de Matos, L.P.; da Silva, V.M.; de Oliveira, J.A. Exogenous jasmonic acid enhances oxidative protection of Lemna valdiviana subjected to arsenic. Acta Physiol. Plant. 2020, 42, 97. [Google Scholar] [CrossRef] [Scilit]
- Yadav, P.; Srivastava, S.; Patil, T.; Raghuvanshi, R.; Srivastava, A.K.; Suprasanna, P. Tracking the time-dependent and tissue-specific processes of arsenic accumulation and stress responses in rice (Oryza sativa L.). J. Hazard. Mater. 2021, 406, 124307. [Google Scholar] [CrossRef] [Scilit]
- Meharg, A.A.; Hartley-Whitaker, J. Arsenic uptake and metabolism in arsenic resistant and nonresistant plant species. New Phytol. 2002, 154, 29–43. [Google Scholar] [CrossRef] [Scilit]
- Meadows, R. How plants control arsenic accumulation. PLoS Biol. 2014, 12, e1002008. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Koch, I.; Wang, L.; Ollson, C.A.; Cullen, W.R.; Reimer, K.J. The predominance of inorganic arsenic species in plants from Yellowknife, northwest territories, Canada. Environ. Sci. Technol. 2000, 34, 22–26. [Google Scholar] [CrossRef] [Scilit]
- Delnomdedieu, M.; Basti, M.M.; Otvos, J.D.; Thomas, D.J. Reduction and binding of arsenate and dimethylarsinate by glutathione: A magnetic resonance study. Chem. Biol. Interact. 1994, 90, 139–155. [Google Scholar] [CrossRef] [Scilit]
- Ströher, E.; Grassl, J.; Carrie, C.; Fenske, R.; Whelan, J.; Millar, A.H. Glutaredoxin S15 is involved in Fe-S cluster transfer in mitochondria influencing lipoic acid-dependent enzymes, plant growth, and arsenic tolerance in Arabidopsis. Plant Physiol. 2016, 170, 1284–1299. [Google Scholar] [CrossRef] [Scilit]
- Van Breusegem, F.; Dat, J.F. Reactive oxygen species in plant cell death. Plant Physiol. 2006, 141, 384–390. [Google Scholar] [CrossRef] [Scilit]
- Talukdar, D. Arsenic-induced changes in growth and antioxidant metabolism of fenugreek. Russ. J. Plant Physiol. 2013, 60, 652–660. [Google Scholar] [CrossRef] [Scilit]
- Chandrakar, V.; Dubey, A.; Keshavkant, S. Modulation of antioxidant enzymes by salicylic acid in arsenic exposed Glycine max L. J. Soil Sci. Plant Nutr. 2016, 16, 662–676. [Google Scholar] [CrossRef] [Scilit]
- Chandrakar, V.; Yadu, B.; Meena, R.K.; Dubey, A.; Keshavkant, S. Arsenic-induced genotoxic responses and their amelioration by diphenylene iodonium, 24-epibrassinolide and proline in Glycine max L. Plant Physiol. Biochem. 2017, 112, 74–86. [Google Scholar] [CrossRef] [Scilit]
- Mucha, S.; Berezowski, M.; Markowska, K. Mechanisms of arsenic toxicity and transport in microorganisms. Adv. Microbiol. 2019, 56, 88–89. [Google Scholar] [CrossRef] [Scilit]
- Gupta, P.; Seth, C.S. Nitrate supplementation attenuates As(V) toxicity in Solanum lycopersicum L. cv Pusa Rohini: Insights into As(V) sub-cellular distribution, photosynthesis, nitrogen assimilation, and DNA damage. Plant Physiol. Biochem. 2019, 139, 44–55. [Google Scholar] [CrossRef] [Scilit]
- Dho, S.; Camusso, W.; Mucciarelli, M.; Fusconi, A. Arsenate toxicity on the apices of Pisum sativum L. seedling roots: Effects on mitotic activity, chromatin integrity and microtubules. Environ. Exp. Bot. 2010, 69, 17–23. [Google Scholar] [CrossRef] [Scilit]
- Tsukagoshi, H. Defective root growth triggered by oxidative stress is controlled through the expression of cell cycle-related genes. Plant Sci. 2012, 197, 30–39. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gupta, K.; Mishra, K.; Srivastava, S.; Kumar, A. Cytotoxic assessment of chromium and arsenic using chromosomal behavior of root meristem in Allium cepa L. Bull. Environ. Contam. Toxicol. 2018, 100, 803–808. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, Z.; Yue, H.; Xing, D. MAP Kinase 6-mediated activation of vacuolar processing enzyme modulates heat shock-induced programmed cell death in Arabidopsis. New Phytol. 2012, 195, 85–96. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Piacentini, D.; Corpas, F.J.; D’Angeli, S.; Altamura, M.M.; Falasca, G. Cadmium and arsenic-induced-stress differentially modulates Arabidopsis root architecture, peroxisome distribution, enzymatic activities and their nitric oxide content. Plant Physiol. Biochem. 2020, 148, 312–323. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sharma, I. Arsenic induced oxidative stress in plants. Biologia 2012, 67, 447–453. [Google Scholar] [CrossRef]
- Devireddy, A.R.; Zandalinas, S.I.; Fichman, Y.; Mittler, R. Integration of reactive oxygen species and hormone signaling during abiotic stress. Plant J. 2021, 105, 459–476. [Google Scholar] [CrossRef] [Scilit]
- Gautam, A.; Pandey, A.K.; Dubey, R.S. Unravelling molecular mechanisms for enhancing arsenic tolerance in plants: A review. Plant Gene 2020, 23, 100240. [Google Scholar] [CrossRef] [Scilit]
- Islam, E.; Khan, M.T.; Irem, S. Biochemical mechanisms of signaling: Perspectives in plants under arsenic stress. Ecotoxicol. Environ. Saf. 2015, 114, 126–133. [Google Scholar] [CrossRef] [Scilit]
- Wang, P.; Chen, X.; Xu, X.; Lu, C.; Zhang, W.; Zhao, F.J. Arsenate induced chlorosis 1/TRANSLOCON at the outer envolope membrane of chloroplasts 132 protects chloroplasts from arsenic toxicity. Plant Physiol. 2018, 178, 1568–1583. [Google Scholar] [CrossRef] [Scilit]
- Asgher, M.; Ahmed, S.; Sehar, Z.; Gautam, H.; Gandhi, S.G.; Khan, N.A. Hydrogen peroxide modulates activity and expression of antioxidant enzymes and protects photosynthetic activity from arsenic damage in rice (Oryza sativa L.). J. Hazard. Mater. 2021, 401, 123365. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Arikan, B.; Ozfidan-Konakci, C.; Yildiztugay, E.; Zengin, G.; Alp, F.; Elbasan, F. Exogenous hesperidin and chlorogenic acid alleviate oxidative damage induced by arsenic toxicity in Zea mays through regulating the water status, antioxidant capacity, redox balance and fatty acid composition. Environ. Pollut. 2022, 292, 118389. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Alsahli, A.A.; Bhat, J.A.; Alyemeni, M.N.; Ashraf, M.; Ahmad, P. Hydrogen sulfide (H2S) mitigates arsenic (As)-induced toxicity in pea (Pisum sativum L.) plants by regulating osmoregulation, antioxidant defense system, ascorbate glutathione cycle and glyoxalase system. J. Plant Growth Regul. 2021, 40, 2515–2531. [Google Scholar] [CrossRef] [Scilit]
- Li, J.; Zhao, Q.; Xue, B.; Wu, H.; Song, G.; Zhang, X. Arsenic and nutrient absorption characteristics and antioxidant response in different leaves of two ryegrass (Lolium perenne) species under arsenic stress. PLoS ONE 2019, 14, e0225373. [Google Scholar] [CrossRef] [Scilit]
- Kaya, C.; Ashraf, M. Sodium hydrosulfite together with silicon detoxifies arsenic toxicity in tomato plants by modulating the AsA-GSH cycle. Environ. Pollut. 2022, 294, 118608. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Natasha; Shahid, M.; Khalid, S.; Saleem, M. Unrevealing arsenic and lead toxicity and antioxidant response in spinach: A human health perspective. Environ. Geochem. Health 2022, 44, 487–496. [Google Scholar] [CrossRef] [Scilit]
- Demircan, N.; Cucun, G.; Uzilday, B. Mitochondrial alternative oxidase (AOX1a) is required for the mitigation of arsenic-induced oxidative stress in Arabidopsis thaliana. Plant Biotechnol. Rep. 2020, 14, 235–245. [Google Scholar] [CrossRef] [Scilit]
- Farooq, M.A.; Zhang, K.; Islam, F.; Wang, J.; Athar, H.U.R.; Nawaz, A.; Ullah Zafar, Z.; Xu, J.; Zhou, W. Physiological and iTRAQ-based quantitative proteomics analysis of methyl jasmonate-induced tolerance in Brassica napus under arsenic stress. Proteomics 2018, 18, e1700290. [Google Scholar] [CrossRef] [Scilit]
- Das, K.; Roychoudhury, A. Reactive oxygen species (ROS) and response of antioxidants as ROS-scavengers during environmental stress in plants. Front. Environ. Sci. 2014, 2, 53. [Google Scholar] [CrossRef] [Scilit]
- Rajput, V.D.; Harish; Singh, R.K.; Verma, K.K.; Sharma, L.; Quiroz-Figueroa, F.R.; Meena, M.; Gour, V.S.; Minkina, T.; Sushkova, S.; et al. Recent developments in enzymatic antioxidant defence mechanism in plants with special reference to abiotic stress. Biology 2021, 10, 267. [Google Scholar] [CrossRef] [Scilit]
- Singh, R.; Misra, A.N.; Sharma, P. Effect of arsenate toxicity on antioxidant enzymes and expression of nicotianamine synthase in contrasting genotypes of bioenergy crop Ricinus communis. Environ. Sci. Pollut. Res. Int. 2021, 28, 31421–31430. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Marques, D.N.; Stolze, S.C.; Harzen, A.; Nogueira, M.L.; Batagin-Piotto, K.D.; Piotto, F.A.; Mason, C.; Azevedo, R.A.; Nakagami, H. Comparative phosphoproteomic analysis of tomato genotypes with contrasting cadmium tolerance. Plant Cell Rep. 2021, 40, 2001–2008. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ahsan, N.; Lee, D.G.; Alam, I.; Kim, P.J.; Lee, J.J.; Ahn, Y.O.; Kwak, S.S.; Lee, I.J.; Bahk, J.D.; Kang, K.Y.; et al. Comparative proteomic study of arsenic-induced differentially expressed proteins in rice roots reveals glutathione plays a central role during as stress. Proteomics 2008, 8, 3561–3576. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Amna, S.; Qamar, S.; Turab Naqvi, A.A.; Al-Huqail, A.A.; Qureshi, M.I. Role of sulfur in combating arsenic stress through upregulation of important proteins, and in-silico analysis to study the interaction between phosphate transporter (PHO1), arsenic and phosphate in spinach. Plant Physiol. Biochem. 2020, 157, 348–358. [Google Scholar] [CrossRef] [Scilit]
- Chauhan, R.; Awasthi, S.; Indoliya, Y.; Chauhan, A.S.; Mishra, S.; Agrawal, L.; Srivastava, S.; Dwivedi, S.; Singh, P.C.; Mallick, S.; et al. Transcriptome and proteome analyses reveal selenium mediated amelioration of arsenic toxicity in rice (Oryza sativa L.). J. Hazard. Mater. 2020, 390, 122122. [Google Scholar] [CrossRef] [Scilit]
- Dixit, G.; Singh, A.P.; Kumar, A.; Dwivedi, S.; Deeba, F.; Kumar, S.; Suman, S.; Adhikari, B.; Shukla, Y.; Trivedi, P.K.; et al. Sulfur alleviates arsenic toxicity by reducing its accumulation and modulating proteome, amino acids and thiol metabolism in rice leaves. Sci. Rep. 2015, 5, 16205. [Google Scholar] [CrossRef] [Scilit]
- Farooq, M.A.; Hong, Z.; Islam, F.; Noor, Y.; Hannan, F.; Zhang, Y.; Ayyaz, A.; Mwamba, T.M.; Zhou, W.; Song, W. Comprehensive proteomic analysis of arsenic induced toxicity reveals the mechanism of multilevel coordination of efficient defense and energy metabolism in two Brassica napus cultivars. Ecotoxicol. Environ. Saf. 2021, 208, 111744. [Google Scholar] [CrossRef] [Scilit]
- Liu, Y.; Damaris, R.N.; Yang, P. Proteomics analysis identified a DRT protein involved in arsenic resistance in Populus. Plant Cell Rep. 2017, 36, 1855–1869. [Google Scholar] [CrossRef] [Scilit]
- Rai, R.; Pandey, S.; Shrivastava, A.K.; Rai, S.P. Enhanced photosynthesis and carbon metabolism favor arsenic tolerance in Artemisia annua, a medicinal plant as revealed by homology-based proteomics. Int. J. Proteom. 2014, 2014, 163962. [Google Scholar] [CrossRef] [Scilit]
- Requejo, R.; Tena, M. Proteome analysis of maize roots reveals that oxidative stress is a main contributing factor to plant arsenic toxicity. Phytochemistry 2005, 66, 1519–1528. [Google Scholar] [CrossRef] [Scilit]
- Marques, D.N.; Carvalho, M.E.A.; Piotto, F.A.; Batagin-Piotto, K.D.; Nogueira, M.L.; Gaziola, S.A.; Azevedo, R.A. Antioxidant defense response in plants to cadmium stress. In Cadmium Tolerance in Plants: Agronomic, Molecular, Signaling, and Omic Approaches; Hasanuzzaman, M., Narasimha, M., Prasad, M.N.V., Nahar, K., Eds.; Elsevier: Amsterdam, The Netherlands, 2019; pp. 423–461. [Google Scholar]
- Marques, D.N.; Gaziola, S.A.; Azevedo, R.A. Phytochelatins and their relationship with modulation of cadmium tolerance in plants. In Handbook of Bioremediation: Physiological, Molecular and Biotechnological Interventions; Hasanuzzaman, M., Prasad, M.N.V., Eds.; Elsevier: Amsterdam, The Netherlands, 2021; pp. 91–113. [Google Scholar]
- Soares, C.; Carvalho, M.E.A.; Azevedo, R.A.; Fidalgo, F. Plants facing oxidative challenges-a little help from the antioxidant networks. Environ. Exp. Bot. 2019, 161, 4–25. [Google Scholar] [CrossRef] [Scilit]
- Tripathi, R.D.; Tripathi, P.; Dwivedi, S.; Dubey, S.; Chatterjee, S.; Chakrabarty, D.; Trivedi, P.K. Arsenomics: Omics of arsenic metabolism in plants. Front. Physiol. 2012, 3, 275. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tripathi, P.; Tripathi, R.D. Metabolome modulation during arsenic stress in plants. In Plant-Metal Interactions; Srivastava, S., Srivastava, A., Suprasanna, P., Eds.; Springer: Singapore, 2019; pp. 119–140. [Google Scholar]
- Shri, M.; Kumar, S.; Chakrabarty, D.; Trivedi, P.K.; Mallick, S.; Misra, P.; Shukla, D.; Mishra, S.; Srivastava, S.; Tripathi, R.D.; et al. Effect of arsenic on growth, oxidative stress, and antioxidant system in rice seedlings. Ecotoxicol. Environ. Saf. 2009, 72, 1102–1110. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Siddiqui, F.; Tandon, P.K.; Srivastava, S. Arsenite and arsenate impact the oxidative status and antioxidant responses in Ocimum tenuiflorum L. Physiol. Mol. Biol. Plants 2015, 21, 453–458. [Google Scholar] [CrossRef] [Scilit]
- Siddiqui, F.; Tandon, P.K.; Srivastava, S. Analysis of arsenic induced physiological and biochemical responses in a medicinal plant, Withania somnifera. Physiol. Mol. Biol. Plants 2015, 21, 61–69. [Google Scholar] [CrossRef] [Scilit]
- Saha, I.; Hasanuzzaman, M.; Adak, M.K. Abscisic acid priming regulates arsenite toxicity in two contrasting rice (Oryza sativa L.) genotypes through differential functioning of sub1A quantitative trait loci. Environ. Pollut. 2021, 287, 117586. [Google Scholar] [CrossRef] [Scilit]
- Bianucci, E.; Furlan, A.; Tordable, M.D.C.; Hernández, L.E.; Carpena-Ruiz, R.O.; Castro, S. Antioxidant responses of peanut roots exposed to realistic groundwater doses of arsenate: Identification of glutathione S-transferase as a suitable biomarker for metalloid toxicity. Chemosphere 2017, 181, 551–561. [Google Scholar] [CrossRef] [Scilit]
- Leão, G.A.; Oliveira, J.A.; Felipe, R.T.A.; Farnese, F.S.; Gusman, G.S. Anthocyanins, thiols, and antioxidant scavenging enzymes are involved in Lemna gibba tolerance to arsenic. J. Plant Interact. 2013, 9, 143–151. [Google Scholar] [CrossRef] [Scilit]
- Mishra, S.; Jha, A.B.; Dubey, R.S. Arsenite treatment induces oxidative stress, upregulates antioxidant system, and causes phytochelatin synthesis in rice seedlings. Protoplasma 2011, 248, 565–577. [Google Scholar] [CrossRef] [Scilit]
- Leão, G.A.; Oliveia, J.A.; Felipe, R.T.A.; Farnese, F.S. Phytoremediation of arsenic-contaminated water: The role of antioxidant metabolism of Azolla caroliniana Willd. (Salviniales). Acta Bot. Bras. 2017, 31, 161–168. [Google Scholar] [CrossRef] [Scilit]
- Saha, J.; Majumder, B.; Mumtaz, B.; Biswas, A.K. Arsenic-induced oxidative stress and thiol metabolism in two cultivars of rice and its possible reversal by phosphate. Acta Physiol. Plant 2017, 39, 263. [Google Scholar] [CrossRef] [Scilit]
- Anjum, S.A.; Tanveer, M.; Hussain, S.; Shahzad, B.; Ashraf, U.; Fahad, S.; Hassan, W.; Jan, S.; Khan, I.; Saleem, M.F.; et al. Osmoregulation and antioxidant production in maize under combined cadmium and arsenic stress. Environ. Sci. Pollut. Res. Int. 2016, 23, 11864–11875. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dave, R.; Tripathi, R.D.; Dwivedi, S.; Tripathi, P.; Dixit, G.; Sharma, Y.K.; Trivedi, P.K.; Corpas, F.J.; Barroso, J.B.; Chakrabarty, D. Arsenate and arsenite exposure modulate antioxidants and amino acids in contrasting arsenic accumulating rice (Oryza sativa L.) genotypes. J. Hazard. Mater. 2013, 262, 1123–1131. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gupta, M.; Ahmad, M.A. Arsenate induced differential response in rice genotypes. Ecotoxicol. Environ. Saf. 2014, 107, 46–54. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Majumder, B.; Das, S.; Mukhopadhyay, S.; Biswas, A.K. Identification of arsenic-tolerant and arsenic-sensitive rice (Oryza sativa L.) cultivars on the basis of arsenic accumulation assisted stress perception, morpho-biochemical responses, and alteration in genomic template stability. Protoplasma 2019, 256, 193–211. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Majumder, B.; Das, S.; Pal, B.; Biswas, A.K. Evaluation of arsenic induced toxicity based on arsenic accumulation, translocation and its implications on physio-chemical changes and genomic instability in indica rice (Oryza sativa L.) cultivars. Ecotoxicol. Environ. Saf. 2020, 29, 13–34. [Google Scholar] [CrossRef] [Scilit]
- Mallick, S.; Sinam, G.; Sinha, S. Study on arsenate tolerant and sensitive cultivars of Zea mays L.: Differential detoxification mechanism and effect on nutrients status. Ecotoxicol. Environ. Saf. 2011, 74, 1316–1324. [Google Scholar] [CrossRef] [Scilit]
- Mallick, S.; Kumar, N.; Sinha, S.; Dubey, A.K.; Tripathi, R.D.; Srivastav, V. H2O2 pretreated rice seedlings specifically reduces arsenate not arsenite: Difference in nutrient uptake and antioxidant defense response in a contrasting pair of rice cultivars. Physiol. Mol. Biol. Plants 2014, 20, 435–447. [Google Scholar] [CrossRef] [Scilit]
- Srivastava, S.; Srivastava, A.K.; Suprasanna, P.; D’Souza, S.F. Comparative biochemical and transcriptional profiling of two contrasting varieties of Brassica juncea L. in response to arsenic exposure reveals mechanisms of stress perception and tolerance. J. Exp. Bot. 2009, 60, 3419–3431. [Google Scholar] [CrossRef] [Scilit]
- Srivastava, S.; Srivastava, A.K.; Suprasanna, P.; D’Souza, S.F. Comparative antioxidant profiling of tolerant and sensitive varieties of Brassica juncea L. to arsenate and arsenite exposure. Bull. Environ. Contam. Toxicol. 2010, 84, 342–346. [Google Scholar] [CrossRef] [Scilit]
- Tripathi, P.; Singh, R.P.; Sharma, Y.K.; Tripathi, R.D. Arsenite stress variably stimulates pro-oxidant enzymes, anatomical deformities, photosynthetic pigment reduction, and antioxidants in arsenic-tolerant and sensitive rice seedlings. Environ. Toxicol. Chem. 2015, 34, 1562–1571. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Singh, R.; Upadhyay, A.K.; Singh, D.P. Regulation of oxidative stress and mineral nutrient status by selenium in arsenic treated crop plant Oryza sativa. Ecotoxicol. Environ. Saf. 2018, 148, 105–113. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tripathi, D.K.; Rai, P.; Guerriero, G.; Sharma, S.; Corpas, F.J.; Singh, V.P. Silicon induces adventitious root formation in rice under arsenate stress with involvement of nitric oxide and indole-3-acetic acid. J. Exp. Bot. 2021, 72, 4457–4471. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Surgun-Acar, Y.; Zemheri-Navruz, F. 24-Epibrassinolide promotes arsenic tolerance in Arabidopsis thaliana L. by altering stress responses at biochemical and molecular level. J. Plant Physiol. 2019, 238, 12–19. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kaya, C.; Ashraf, M.; Alyemeni, M.N.; Corpas, F.J.; Ahmad, P. Salicylic acid-induced nitric oxide enhances arsenic toxicity tolerance in maize plants by upregulating the ascorbate-glutathione cycle and glyoxalase system. J. Hazard. Mater. 2020, 399, 123020. [Google Scholar] [CrossRef] [Scilit]
- Singh, A.P.; Dixit, G.; Kumar, A.; Mishra, S.; Kumar, N.; Dixit, S.; Singh, P.K.; Dwivedi, S.; Trivedi, P.K.; Pandey, V.; et al. A protective role for nitric oxide and salicylic acid for arsenite phytotoxicity in rice (Oryza sativa L.). Plant Physiol. Biochem. 2017, 115, 163–173. [Google Scholar] [CrossRef] [Scilit]
- Farooq, M.A.; Islam, F.; Yang, C.; Nawaz, A.; Athar, H.R.; Gill, R.A.; Ali, B.; Song, W.; Zhou, W. Methyl jasmonate alleviates arsenic-induced oxidative damage and modulates the ascorbate–glutathione cycle in oilseed rape roots. J. Plant Growth Regul. 2018, 84, 135–148. [Google Scholar] [CrossRef] [Scilit]
- Praveen, A.; Gupta, M. Nitric oxide confronts arsenic stimulated oxidative stress and root architecture through distinct gene expression of auxin transporters, nutrient related genes and modulates biochemical responses in Oryza sativa L. Environ. Pollut. 2019, 240, 950–962. [Google Scholar] [CrossRef] [Scilit]
- Praveen, A.; Pandey, A.; Gupta, M. Nitric oxide alters nitrogen metabolism and PIN gene expressions by playing protective role in arsenic challenged Brassica juncea L. Ecotoxiol. Environ. Saf. 2019, 176, 95–107. [Google Scholar] [CrossRef] [Scilit]
- Kumar, A.; Pal, L.; Agrawal, V. Glutathione and citric acid modulates lead-and arsenic-induced phytotoxicity and genotoxicity responses in two cultivars of Solanum lycopersicum L. Acta Physiol. Plant. 2017, 39, 151. [Google Scholar] [CrossRef] [Scilit]
- Zheng, W.; Zhong, Z.Y.; Wang, H.B.; Wang, H.J.; Wu, D.M. Effects of oxalic acid on arsenic uptake and the physiological responses of Hydrilla verticillata exposed to different forms of arsenic. Bull. Environ. Contam. Toxicol. 2018, 100, 653–658. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Samanta, S.; Banerjee, A.; Roychoudhury, A. Melatonin application differentially modulates the enzymes associated with antioxidative machinery and ascorbate-glutathione cycle during arsenate exposure in indica rice varieties. Plant Biol. 2021, 23, 193–201. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Das, J.; Sarkar, P. Remediation of arsenic in mung bean (Vigna radiata) with growth enhancement by unique arsenic-resistant bacterium Acinetobacter lwoffii. Sci. Total Environ. 2018, 624, 1106–1118. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, X.; Ahammed, G.J.; Zhang, X.N.; Zhang, L.; Yan, P.; Zhang, L.P.; Fu, J.Y.; Han, W.Y. Melatonin-mediated regulation of anthocyanin biosynthesis and antioxidant defense confer tolerance to arsenic stress in Camellia sinensis L. J. Hazard. Mater. 2021, 403, 123922. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dolui, D.; Hasanuzzaman, M.; Saha, I.; Ghosh, A.; Adak, M.K. Amelioration of sodium and arsenic toxicity in Salvinia natans L. with 2, 4-D priming through physiological responses. Environ. Sci. Pollut. Res. 2022, 29, 9232–9247. [Google Scholar] [CrossRef] [Scilit]
- Singh, S.; Husain, T.; Kushwaha, B.K.; Suhel, M.; Fatima, A.; Mishra, V.; Singh, S.K.; Tripathi, D.K.; Rai, M.; Prasad, S.M.; et al. Regulation of ascorbate-glutathione cycle by exogenous nitric oxide and hydrogen peroxide in soybean roots under arsenate stress. J. Hazard. Mater. 2020, 409, 123686. [Google Scholar] [CrossRef] [Scilit]
- Rahman, A.; Mostofa, M.G.; Alam, M.M.; Nahar, K.; Hasanuzzaman, M.; Fujita, M. Calcium mitigates arsenic toxicity in rice seedlings by reducing arsenic uptake and modulating the antioxidant defense and glyoxalase systems and stress markers. BioMed Res. Int. 2015, 2015, 340812. [Google Scholar] [CrossRef] [Scilit]
- Singh, R.; Parihar, P.; Prasad, S.M. Sulphur and calcium attenuate arsenic toxicity in Brassica by adjusting ascorbate–glutathione cycle and sulphur metabolism. J. Plant Growth Regul. 2020, 91, 221–235. [Google Scholar] [CrossRef] [Scilit]
- Rohman, M.M.; Tonny, S.H.; Alam, S.S.; Omy, S.H.; Akhi, A.H.; Raihan, H.U.Z.; Akter, T.; Parvin, K.; Hasanuzzaman, M. Role of phytohormones in antioxidant metabolism in plants under salinity and water stress. In Managing Plant Production under Changing Environment; Hasanuzzaman, M., Ahammed, G.J., Nahar, K., Eds.; Springer: Singapore, 2022; pp. 151–191. [Google Scholar]
- Farooq, M.A.; Gill, R.A.; Islam, F.; Ali, B.; Liu, H.; Xu, J.; He, S.; Zhou, W. Methyl jasmonate regulates antioxidant defense and suppresses arsenic uptake in Brassica napus L. Front. Plant Sci. 2016, 7, 468. [Google Scholar] [CrossRef] [Scilit]
- Verma, G.; Srivastava, D.; Narayan, S.; Shirke, P.A.; Chakrabarty, D. Exogenous application of methyl jasmonate alleviates arsenic toxicity by modulating its uptake and translocation in rice (Oryza sativa L.). Ecotoxicol. Environ. Saf. 2020, 201, 110735. [Google Scholar] [CrossRef] [Scilit]
- Mousavi, S.R.; Niknejad, Y.; Fallah, H.; Tari, D.B. Methyl jasmonate alleviates arsenic toxicity in rice. Plant Cell Rep. 2020, 39, 1041–1060. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, H.; Cui, S.; Wu, D.; Yang, X.; Wang, H.; Wang, Z. Effects of kinetin on arsenic speciation and antioxidative enzymes in fronds of the arsenic hyperaccumulator Pteris cretica var. nervosa and non-hyperaccumulator Pteris ensiformis. Environ. Exp. Bot. 2021, 191, 104622. [Google Scholar] [CrossRef] [Scilit]
- Singh, M.; Singh, V.P.; Dubey, G.; Prasad, S.M. Exogenous proline application ameliorates toxic effects of arsenate in Solanum melongena L. seedlings. Ecotoxicol. Environ. Saf. 2015, 117, 164–173. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Da-Silva, C.J.; Canatto, R.A.; Cardoso, A.A.; Ribeiro, C.; de Oliveira, J.A. Oxidative stress triggered by arsenic in a tropical macrophyte is alleviated by endogenous and exogenous nitric oxide. Braz. J. Bot. 2018, 41, 21–28. [Google Scholar] [CrossRef] [Scilit]
- Ghorbani, A.; Pishkar, L.; Roodbari, N.; Pehlivan, N.; Wu, C. Nitric oxide could allay arsenic phytotoxicity in tomato (Solanum lycopersicum L.) by modulating photosynthetic pigments, phytochelatin metabolism, molecular redox status and arsenic sequestration. Plant Physiol. Biochem. 2021, 167, 337–348. [Google Scholar] [CrossRef] [Scilit]
- Ghorbani, A.; Pishkar, L.; Roodbari, N.; Tavakoli, S.A.; Jahromi, E.M.; Wu, C. Nitrate reductase is needed for methyl jasmonate-mediated arsenic toxicity tolerance of rice by modulating the antioxidant defense system, glyoxalase system and arsenic sequestration mechanism. J. Plant Growth Regul. 2022, 1–13. [Google Scholar] [CrossRef] [Scilit]
- Bhat, J.A.; Bhat, M.A.; Abdalmegeed, D.; Yu, D.; Chen, J.; Bajguz, A.; Ahmad, A.; Ahmad, P. Newly-synthesized iron-oxide nanoparticles showed synergetic effect with citric acid for alleviating arsenic phytotoxicity in soybean. Environ. Pollut. 2021, 295, 118693. [Google Scholar] [CrossRef] [Scilit]
- Shahid, M.; Rafiq, M.; Niazi, N.K.; Dumat, C.; Shamshad, S.; Khalid, S.; Bibi, I. Arsenic accumulation and physiological attributes of spinach in the presence of amendments: An implication to reduce health risk. Environ. Sci. Pollut. Res. 2017, 24, 16097–16106. [Google Scholar] [CrossRef] [Scilit]
- Rafiq, M.; Shahid, M.; Abbas, G.; Shamshad, S.; Khalid, S.; Niazi, N.K.; Dumat, C. Comparative effect of calcium and EDTA on arsenic uptake and physiological attributes of Pisum sativum. Int. J. Phytoremediat. 2017, 19, 662–669. [Google Scholar] [CrossRef] [Scilit]
- Hakeem, K.R.; Alharby, H.F.; Bamagoos, A.A.; Pirzadah, T.B. Biochar promotes arsenic (As) immobilization in contaminated soils and alleviates the As-toxicity in soybean (Glycine max (L.) Merr.). Chemosphere 2022, 292, 133407. [Google Scholar] [CrossRef] [Scilit]
- Kamran, M.A.; Bibi, S.; Chen, B. Preventative effect of crop straw-derived biochar on plant growth in an arsenic polluted acidic ultisol. Sci. Total Environ. 2021, 812, 151469. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xiao, A.W.; Li, Z.; Li, W.C.; Ye, Z.H. The effect of plant growth-promoting rhizobacteria (PGPR) on arsenic accumulation and the growth of rice plants (Oryza sativa L.). Chemosphere 2020, 242, 125136. [Google Scholar]
- Mondal, S.; Pramanik, K.; Ghosh, S.K.; Pal, P.; Mondal, T.; Soren, T.; Maiti, T.K. Unraveling the role of plant growth-promoting rhizobacteria in the alleviation of arsenic phytotoxicity: A review. Microbiol. Res. 2021, 250, 126809. [Google Scholar] [CrossRef] [Scilit]
- Pandey, N.; Bhatt, R. Role of soil associated Exiguobacterium in reducing arsenic toxicity and promoting plant growth in Vigna radiata. Eur. J. Soil Biol. 2016, 75, 142–150. [Google Scholar] [CrossRef] [Scilit]
- Pandey, S.; Ghosh, P.K.; Ghosh, S.; De, T.K.; Maiti, T.K. Role of heavy metal resistant Ochrobactrum sp. and Bacillus spp. strains in bioremediation of a rice cultivar and their PGPR like activities. J. Microbiol. 2013, 51, 11–17. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, Q.; Xiong, D.; Zhao, P.; Yu, X.; Tu, B.; Wang, G. Effect of applying an arsenic-resistant and plant growth–promoting rhizobacterium to enhance soil arsenic phytoremediation by Populus deltoides LH05-17. J. Appl. Microbiol. 2011, 111, 1065–1074. [Google Scholar] [CrossRef] [Scilit]
- Pinter, I.F.; Salomon, M.V.; Berli, F.; Bottini, R.; Piccoli, P. Characterization of the As (III) tolerance conferred by plant growth promoting rhizobacteria to in vitro-grown grapevine. Appl. Soil Ecol. 2017, 109, 60–68. [Google Scholar] [CrossRef] [Scilit]
- Ghosh, P.K.; Maiti, T.K.; Pramanik, K.; Ghosh, S.K.; Mitra, S.; De, T.K. The role of arsenic resistant Bacillus aryabhattai MCC3374 in promotion of rice seedlings growth and alleviation of arsenic phytotoxicity. Chemosphere 2018, 211, 407–419. [Google Scholar] [CrossRef] [Scilit]
- Soto, J.; Ortiz, J.; Herrera, H.; Fuentes, A.; Almonacid, L.; Charles, T.C.; Arriagada, C. Enhanced arsenic tolerance in Triticum aestivum inoculated with arsenic-resistant and plant growth promoter microorganisms from a heavy metal-polluted soil. Microorganisms 2019, 7, 348. [Google Scholar] [CrossRef] [Scilit]
- Ghosh, A.; Pramanik, K.; Bhattacharya, S.; Mondal, S.; Ghosh, S.K.; Ghosh, P.K.; Maiti, T.K. Abatement of arsenic-induced phytotoxic effects in rice seedlings by an arsenic-resistant Pantoea dispersa strain. Environ. Sci. Pollut. Res. 2021, 28, 21633–21649. [Google Scholar] [CrossRef] [Scilit]
- Ghorbani, A.; Tafteh, M.; Roudbari, N.; Pishkar, L.; Zhang, W.; Wu, C. Piriformospora indica augments arsenic tolerance in rice (Oryza sativa) by immobilizing arsenic in roots and improving iron translocation to shoots. Ecotoxicol. Environ. Saf. 2021, 209, 111793. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nawaz, M.A.; Jiao, Y.; Chen, C.; Shireen, F.; Zheng, Z.; Imtiaz, M.; Bie, Z.; Huang, Y. Melatonin pretreatment improves vanadium stress tolerance of watermelon seedlings by reducing vanadium concentration in the leaves and regulating melatonin biosynthesis and antioxidant-related gene expression. J. Plant Physiol. 2018, 220, 115–127. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Farouk, S.; Al-Amri, S.M. Exogenous melatonin-mediated modulation of arsenic tolerance with improved accretion of secondary metabolite production, activating antioxidant capacity and improved chloroplast ultrastructure in rosemary herb. Ecotoxicol. Environ. Saf. 2019, 180, 333–347. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Samanta, S.; Banerjee, A.; Roychoudhury, A. Arsenic toxicity is counteracted by exogenous application of melatonin to different extents in arsenic-susceptible and arsenic-tolerant rice cultivars. J. Plant Growth Regul. 2021. [Google Scholar] [CrossRef] [Scilit]
- Jung, H.I.; Kong, M.S.; Chae, M.J.; Lee, E.J.; Jung, G.B.; Kim, Y.H. Effect of ascorbate on the arsenic uptake, ROS-scavenging capacity, and antioxidant homeostasis in rice. Korean J. Soil Sci. Fertil. 2018, 51, 90–100. [Google Scholar] [CrossRef] [Scilit]
- Jung, H.; Kong, M.S.; Lee, B.R.; Kim, T.H.; Chae, M.J.; Lee, E.J.; Jung, G.B.; Lee, C.H.; Sung, J.K.; Kim, Y.H. Exogenous glutathione increases arsenic translocation into shoots and alleviates arsenic-induced oxidative stress by sustaining ascorbate–glutathione homeostasis in rice seedlings. Front. Plant Sci. 2019, 10, 1089. [Google Scholar] [CrossRef] [Scilit]
- Jiang, M.; Song, Y.; Kanwar, M.K.; Ahammed, G.J.; Shao, S.; Zhou, J. Phytonanotechnology applications in modern agriculture. J. Nanobiotechnol. 2021, 19, 430. [Google Scholar] [CrossRef] [Scilit]
- Singh, A.; Tiwari, S.; Pandey, J.; Lata, C.; Singh, I.K. Role of nanoparticles in crop improvement and abiotic stress management. J. Biotechnol. 2021, 337, 57–70. [Google Scholar] [CrossRef] [Scilit]
- Bidi, H.; Fallah, H.; Niknejad, Y.; Barari Tari, D. Iron oxide nanoparticles alleviate arsenic phytotoxicity in rice by improving iron uptake, oxidative stress tolerance and diminishing arsenic accumulation. Plant Physiol. Biochem. 2021, 163, 348–357. [Google Scholar] [CrossRef] [Scilit]
- Yan, S.; Wu, F.; Zhou, S.; Yang, J.; Tang, X.; Ye, W. Zinc oxide nanoparticles alleviate the arsenic toxicity and decrease the accumulation of arsenic in rice (Oryza sativa L.). BMC Plant Biol. 2021, 21, 150. [Google Scholar] [CrossRef] [Scilit]
- Kiany, T.; Pishkar, L.; Sartipnia, N.; Iranbakhsh, A.; Barzin, G. Effects of silicon and titanium dioxide nanoparticles on arsenic accumulation, phytochelatin metabolism, and antioxidant system by rice under arsenic toxicity. Environ. Sci. Pollut. Res. 2022. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zeeshan, M.; Hu, Y.X.; Iqbal, A.; Salam, A.; Liu, Y.X.; Muhammad, I.; Ahmad, S.; Khan, A.H.; Hale, B.; Wu, H.Y.; et al. Amelioration of AsV toxicity by concurrent application of ZnO-NPs and Se-NPs is associated with differential regulation of photosynthetic indexes, antioxidant pool and osmolytes content in soybean seedling. Ecotoxicol. Environ. Saf. 2021, 225, 112738. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tripathi, D.K.; Singh, S.; Singh, V.P.; Prasad, S.M.; Chauhan, D.K.; Dubey, N.K. Silicon nanoparticles more efficiently alleviate arsenate toxicity than silicon in maize cultiver and hybrid differing in arsenate tolerance. Front. Environ. Sci. 2016, 4, 46. [Google Scholar] [CrossRef] [Scilit]
- González-Moscoso, M.; Juárez-Maldonado, A.; Cadenas-Pliego, G.; Meza-Figueroa, D.; SenGupta, B.; Martínez-Villegas, N. Silicon nanoparticles decrease arsenic translocation and mitigate phytotoxicity in tomato plants. Environ. Sci. Pollut. Res. Int. 2022, 1–17. [Google Scholar] [CrossRef] [Scilit]
- Shabnam, N.; Kim, M.; Kim, H. Iron (III) oxide nanoparticles alleviate arsenic induced stunting in Vigna radiata. Ecotoxicol. Environ. Saf. 2019, 183, 109496. [Google Scholar] [CrossRef] [Scilit]
- Yang, J.; Gao, M.X.; Hu, H.; Ding, X.M.; Lin, H.W.; Wang, L.; Xu, J.M.; Mao, C.Z.; Zhao, F.J.; Wu, Z.C. OsCLT1, a CRT-like transporter 1, is required for glutathione homeostasis and arsenic tolerance in rice. New Phytol. 2016, 211, 658–670. [Google Scholar] [CrossRef] [Scilit]
- Yu, G.; Wang, X.; Liu, J.; Jian, P.; You, S.; Ding, N.; Guo, Q.; Lin, F. Applications of nanomaterials for heavy metal removal from water and soil: A review. Sustainability 2021, 13, 713. [Google Scholar] [CrossRef] [Scilit]
- Kandhol, N.; Aggarwal, B.; Bansal, R.; Parveen, N.; Singh, V.P.; Chauhan, D.K.; Sonah, H.; Sahi, S.; Grillo, R.; Peralta-Videa, J.; et al. Nanoparticles as a potential protective agent for arsenic toxicity alleviation in plants. Environ. Pollut. 2022, 300, 118887. [Google Scholar] [CrossRef] [Scilit]
- Wu, F.; Fang, Q.; Yan, S.; Pan, L.; Tang, X.; Ye, W. Effects of zinc oxide nanoparticles on arsenic stress in rice (Oryza sativa L.): Germination, early growth, and arsenic uptake. Environ. Sci. Pollut. Res. 2020, 27, 26974–26981. [Google Scholar] [CrossRef] [Scilit]
- Srivastava, S.; Suprasanna, P.; D’souza, S.F. Mechanisms of arsenic tolerance and detoxification in plants and their application in transgenic technology: A critical appraisal. Int. J. Phytoremediat. 2012, 14, 506–517. [Google Scholar] [CrossRef] [Scilit]
- Kumari, P.; Rastogi, A.; Shukla, A.; Srivastava, S.; Yadav, S. Prospects of genetic engineering utilizing potential genes for regulating arsenic accumulation in plants. Chemosphere 2018, 211, 397–406. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Awasthi, S.; Chauhan, R.; Srivastava, S.; Tripathi, R.D. The journey of arsenic from soil to grain in rice. Front. Plant Sci. 2017, 8, 1007. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sanchez-Bermejo, E.; Castrillo, G.; Del Llano, B.; Navarro, C.; Zarco-Fernandez, S.; Martinez-Herrera, D.J.; Leo-del Puerto, Y.; Munoz, R.; Camara, C.; Paz-Ares, J.; et al. Natural variation in arsenate tolerance identifies an arsenate reductase in Arabidopsis thaliana. Nat. Commun. 2014, 5, 4617. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chao, D.Y.; Chen, Y.; Chen, J.; Shi, S.; Chen, Z.; Wang, C. Genome-wide association mapping identifies a new arsenate reductase enzyme critical for limiting arsenic accumulation in plants. PLoS Biol. 2014, 12, e1002009. [Google Scholar] [CrossRef] [Scilit]
- Xu, J.; Shi, S.; Wang, L.; Tang, Z.; Lv, T.; Zhu, X. OsHAC4 is critical for arsenate tolerance and regulates arsenic accumulation in rice. New Phytol. 2017, 215, 1090–1101. [Google Scholar] [CrossRef] [Scilit]
- Sundaram, S.; Wu, S.; Ma, L.Q.; Rathinasabapathi, B. Expression of a Pteris vittate glutaredoxin PvGRX5 in transgenic Arabidopsis thaliana increases plant arsenic tolerance and decreases arsenic accumulation in the leaves. Plant Cell Environ. 2009, 32, 851–858. [Google Scholar] [CrossRef] [Scilit]
- Khan, M.I.R.; Chopra, P.; Chhillar, H.; Ahanger, M.A.; Hussain, S.J.; Maheshwari, C. Regulatory hubs and strategies for improving heavy metal tolerance in plants: Chemical messengers, omics and genetic engineering. Plant Physiol. Biochem. 2021, 164, 260–278. [Google Scholar] [CrossRef] [Scilit]
- Kumar, S.; Trivedi, P.K. Glutathione S-transferases: Role in combating abiotic stresses including arsenic detoxification in plants. Front. Plant Sci. 2018, 9, 751. [Google Scholar] [CrossRef] [Scilit]
- Yadav, S.K. Heavy metals toxicity in plants: An overview on the role of glutathione and phytochelatins in heavy metal stress tolerance of plants. S. Afr. J. Bot. 2010, 76, 167–179. [Google Scholar] [CrossRef] [Scilit]
- Ronzan, M.; Zanella, L.; Fattorini, L.; Della Rovere, F.; Urgast, D.; Cantamessa, S.; Nigro, A.; Barbieri, M.; Sanità di Toppi, L.; Berta, G.; et al. The morphogenic responses and phytochelatin complexes induced by arsenic in Pteris vittata change in the presence of cadmium. Environ. Exp. Bot. 2017, 133, 176–187. [Google Scholar] [CrossRef] [Scilit]
- Pathare, V.; Srivastava, S.; Suprasanna, P. Evaluation of effects of arsenic on carbon, nitrogen and sulphur metabolism in two contrasting varieties of Brassica juncea. Acta Physiol. Plant. 2013, 35, 3377–3389. [Google Scholar] [CrossRef] [Scilit]
- Chen, J.; Yang, L.; Yan, X.; Liu, Y.; Wang, R.; Fan, T.; Ren, Y.; Tang, X.; Xiao, F.; Liu, Y.; et al. Zinc-Finger transcription factor ZAT6 positively regulates cadmium tolerance through the glutathione-dependent pathway in Arabidopsis. Plant Physiol. 2016, 171, 707–719. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Khare, D.; Mitsuda, N.; Lee, S.; Song, W.Y.; Hwang, D.; Ohme-Takagi, M.; Hwang, J.U. Root avoidance of toxic metals requires the GeBP-LIKE 4 transcription factor in Arabidopsis thaliana. New Phytol. 2017, 213, 1257–1273. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yuce, M.; Taspinar, M.S.; Aydin, M.; Agar, G. Response of NAC transcription factor genes against chromium stress in sunflower (Helianthus annuus L.). Plant Cell Tissue Organ Cult. 2019, 136, 479–487. [Google Scholar] [CrossRef] [Scilit]
- Zhang, P.; Wang, R.; Ju, Q.; Li, W.; Tran, L.S.P.; Xu, J. The R2R3-MYB transcription factor MYB49 regulates cadmium accumulation. Plant Physiol. 2019, 180, 529–542. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, C.; Zhang, Y.; Liu, Y.; Xu, H.; Zhang, T.; Hu, Z.; Lou, L.; Cai, Q. Ectopic expression of wheat aquaglyceroporin TaNIP2; 1 alters arsenic accumulation and tolerance in Arabidopsis thaliana. Ecotoxicol. Environ. Saf. 2020, 205, 111131. [Google Scholar] [CrossRef] [Scilit]
- Manuka, R.; Saddhe, A.A.; Srivastava, A.K.; Kumar, K.; Penna, S. Overexpression of rice OsWNK9 promotes arsenite tolerance in transgenic Arabidopsis plants. J. Biotechnol. 2021, 332, 114–125. [Google Scholar] [CrossRef] [Scilit]
- Kidwai, M.; Dhar, Y.V.; Gautam, N.; Tiwari, M.; Ahmad, I.Z.; Asif, M.H.; Chakrabarty, D. Oryza sativa class III peroxidase (OsPRX38) overexpression in Arabidopsis thaliana reduces arsenic accumulation due to apoplastic lignification. J. Hazard. Mater. 2019, 362, 383–393. [Google Scholar] [CrossRef] [Scilit]
- Verma, P.K.; Verma, S.; Pande, V.; Mallick, S.; Deo Tripathi, R.; Dhankher, O.P.; Chakrabarty, D. Overexpression of rice glutaredoxin OsGrx_C7 and OsGrx_C2.1 reduces intracellular arsenic accumulation and increases tolerance in Arabidopsis thaliana. Front. Plant Sci. 2016, 7, 740. [Google Scholar] [CrossRef] [Scilit]
- Zanella, L.; Fattorini, L.; Brunetti, P.; Roccotiello, E.; Cornara, L.; D’Angeli, S.; Della Rovere, F.; Cardarelli, M.; Barbieri, M.; Sanita di Toppi, L.; et al. Overexpression of AtPCS1 in tobacco increases arsenic and arsenic plus cadmium accumulation and detoxification. Planta 2016, 243, 605–622. [Google Scholar] [CrossRef] [Scilit]
- Chen, Y.; Wang, H.Y.; Chen, Y.F. The transcription factor MYB40 is a central regulator in arsenic resistance in Arabidopsis. Plant Commun. 2021, 2, 100234. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tiwari, M.; Kidwai, M.; Dutta, P.; Narayan, S.; Gautam, N.; Chawda, K.; Shirke, P.A.; Mishra, A.K.; Chakrabarty, D. A tau class glutathione-S-transferase (OsGSTU5) confers tolerance against arsenic toxicity in rice by accumulating more arsenic in root. J. Hazard. Mater. 2022, 426, 128100. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nishida, S.; Duan, G.; Ohkama-Ohtsu, N.; Uraguchi, S.; Fujiwara, T. Enhanced arsenic sensitivity with excess phytochelatin accumulation in shoots of a SULTR1; 2 knockout mutant of Arabidopsis thaliana (L.) Heynh. Soil Sci. Plant Nutr. 2016, 62, 367–372. [Google Scholar] [CrossRef] [Scilit]
- Luan, M.; Liu, J.; Liu, Y.; Han, X.; Sun, G.; Lan, W.; Luan, S. Vacuolar phosphate transporter 1 (VPT1) affects arsenate tolerance by regulating phosphate homeostasis in Arabidopsis. Plant Cell Physiol. 2018, 59, 1345–1352. [Google Scholar] [CrossRef] [Scilit]
- Kim, D.; Bahmani, R.; Modareszadeh, M.; Hwang, S. Mechanism for higher tolerance to and lower accumulation of arsenite in NtCyc07-overexpressing tobacco. Plants 2020, 9, 1480. [Google Scholar] [CrossRef] [Scilit]
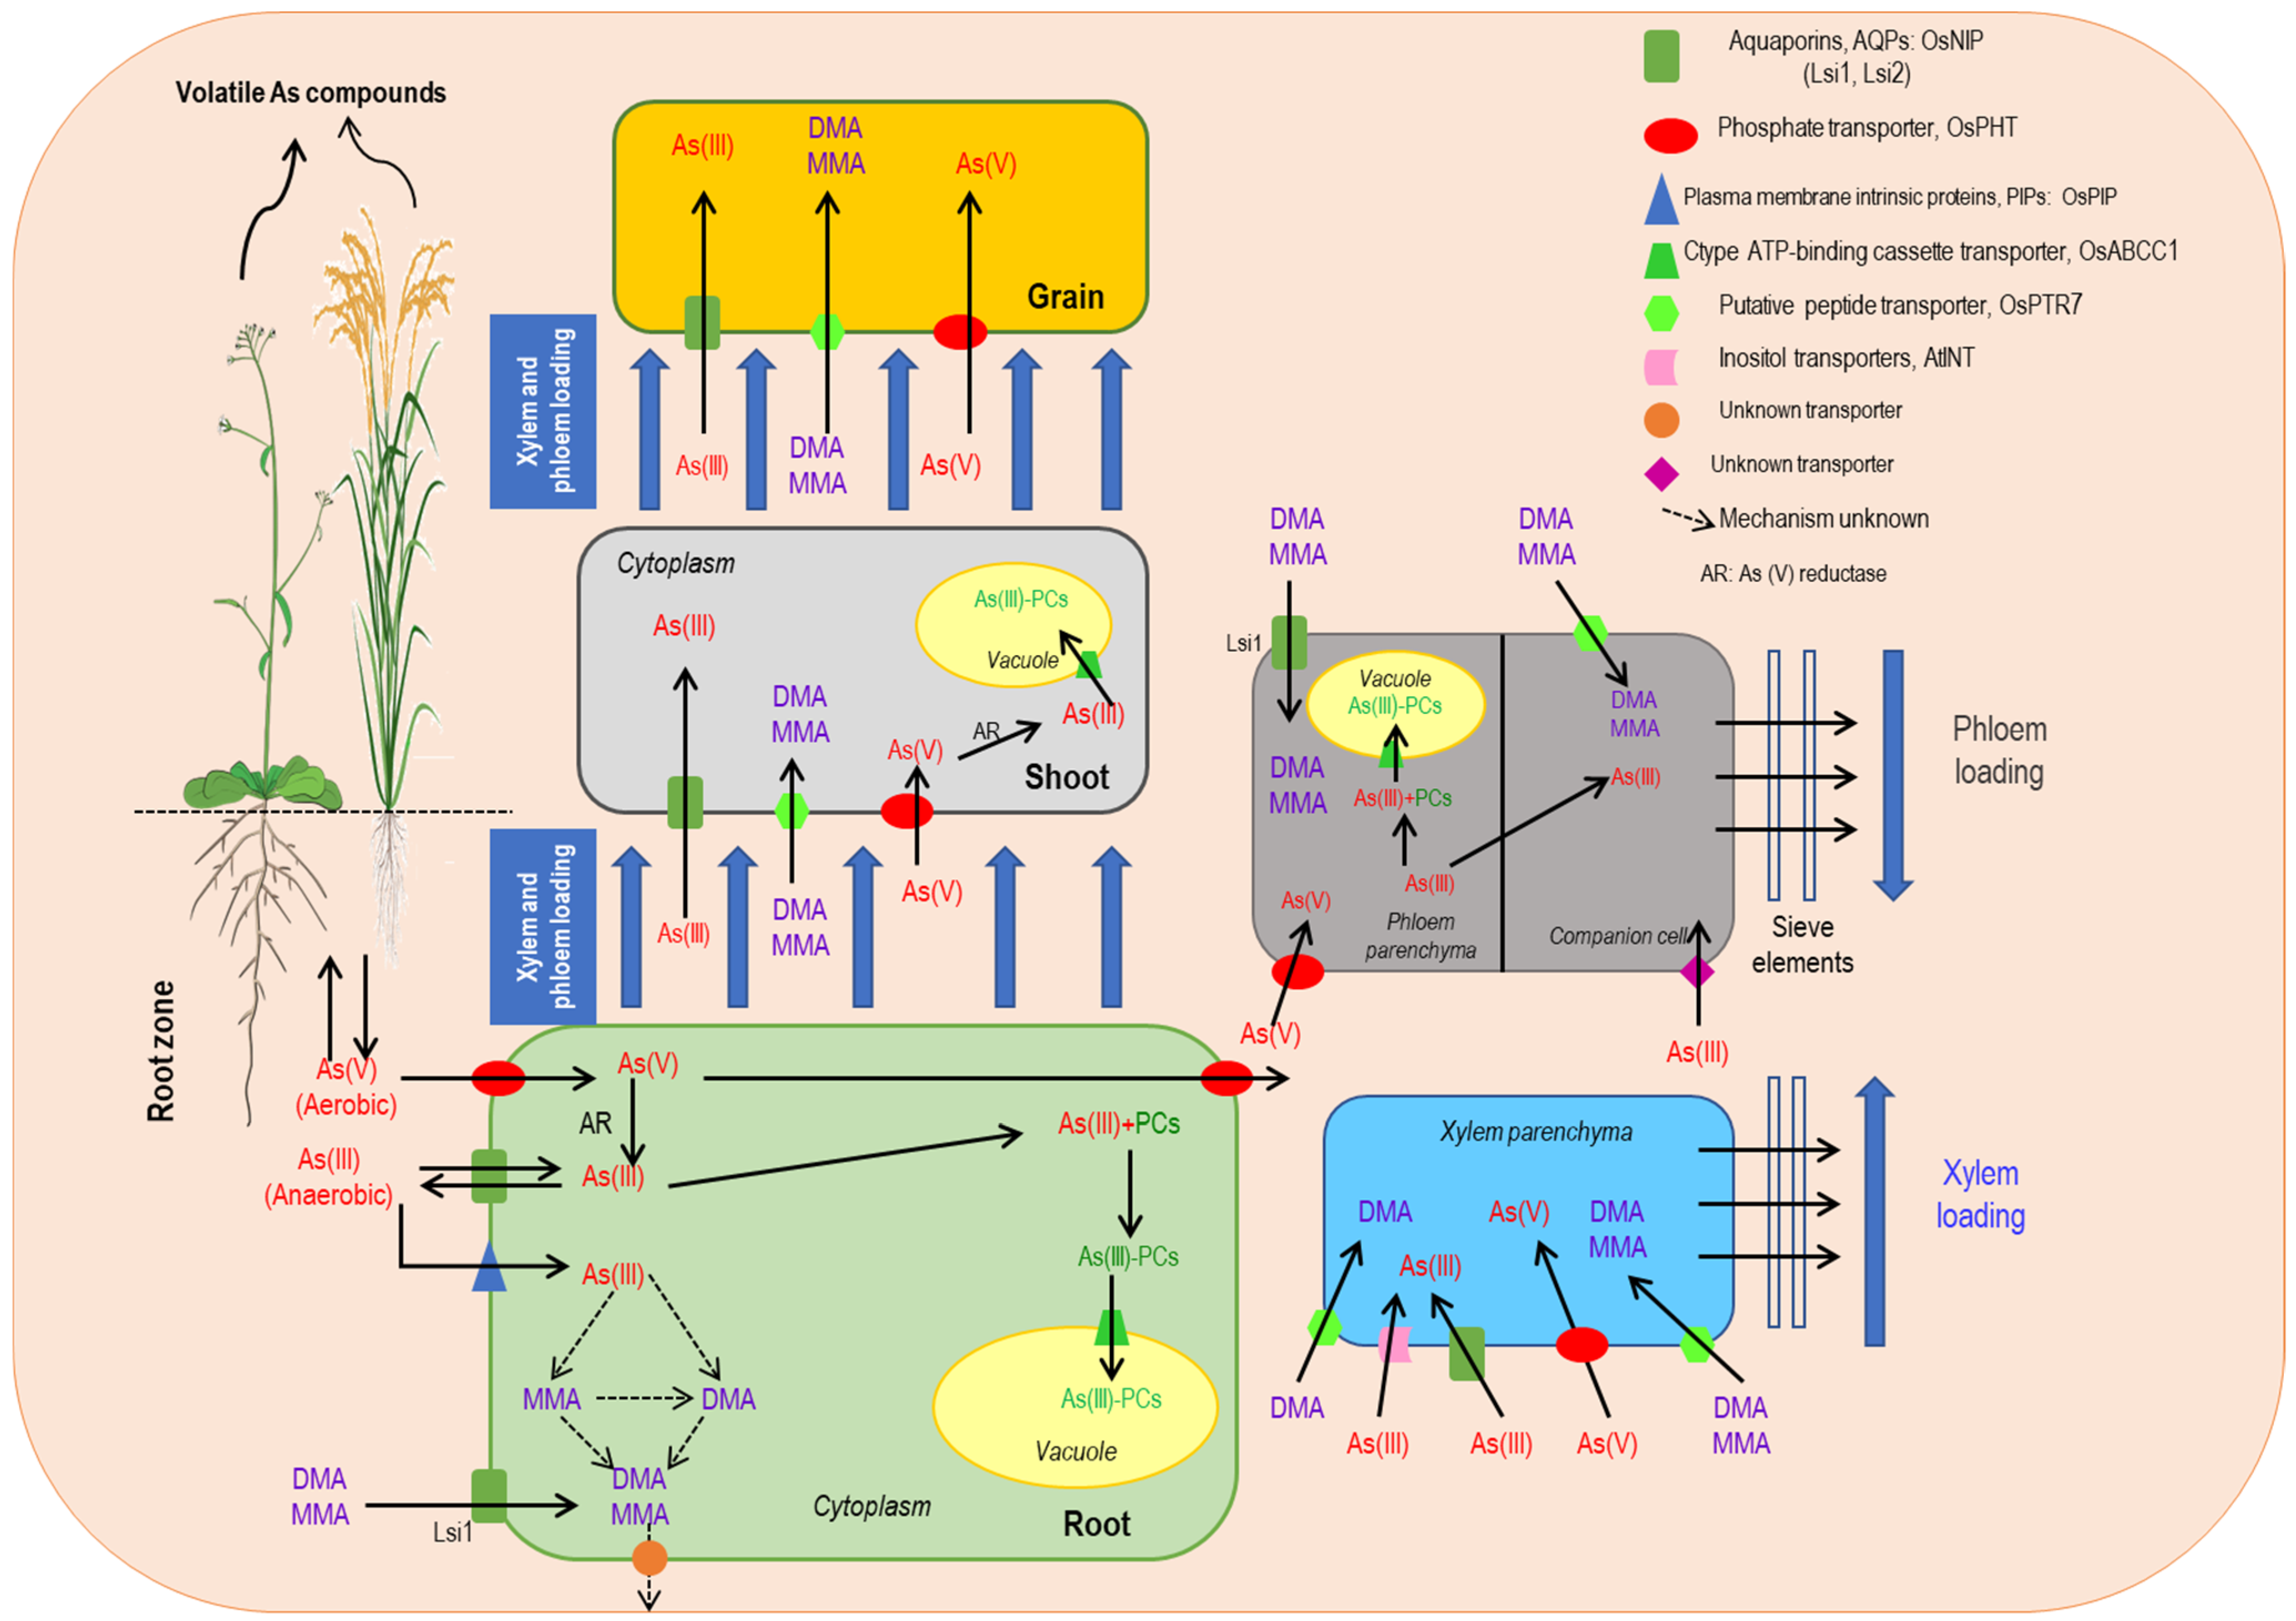
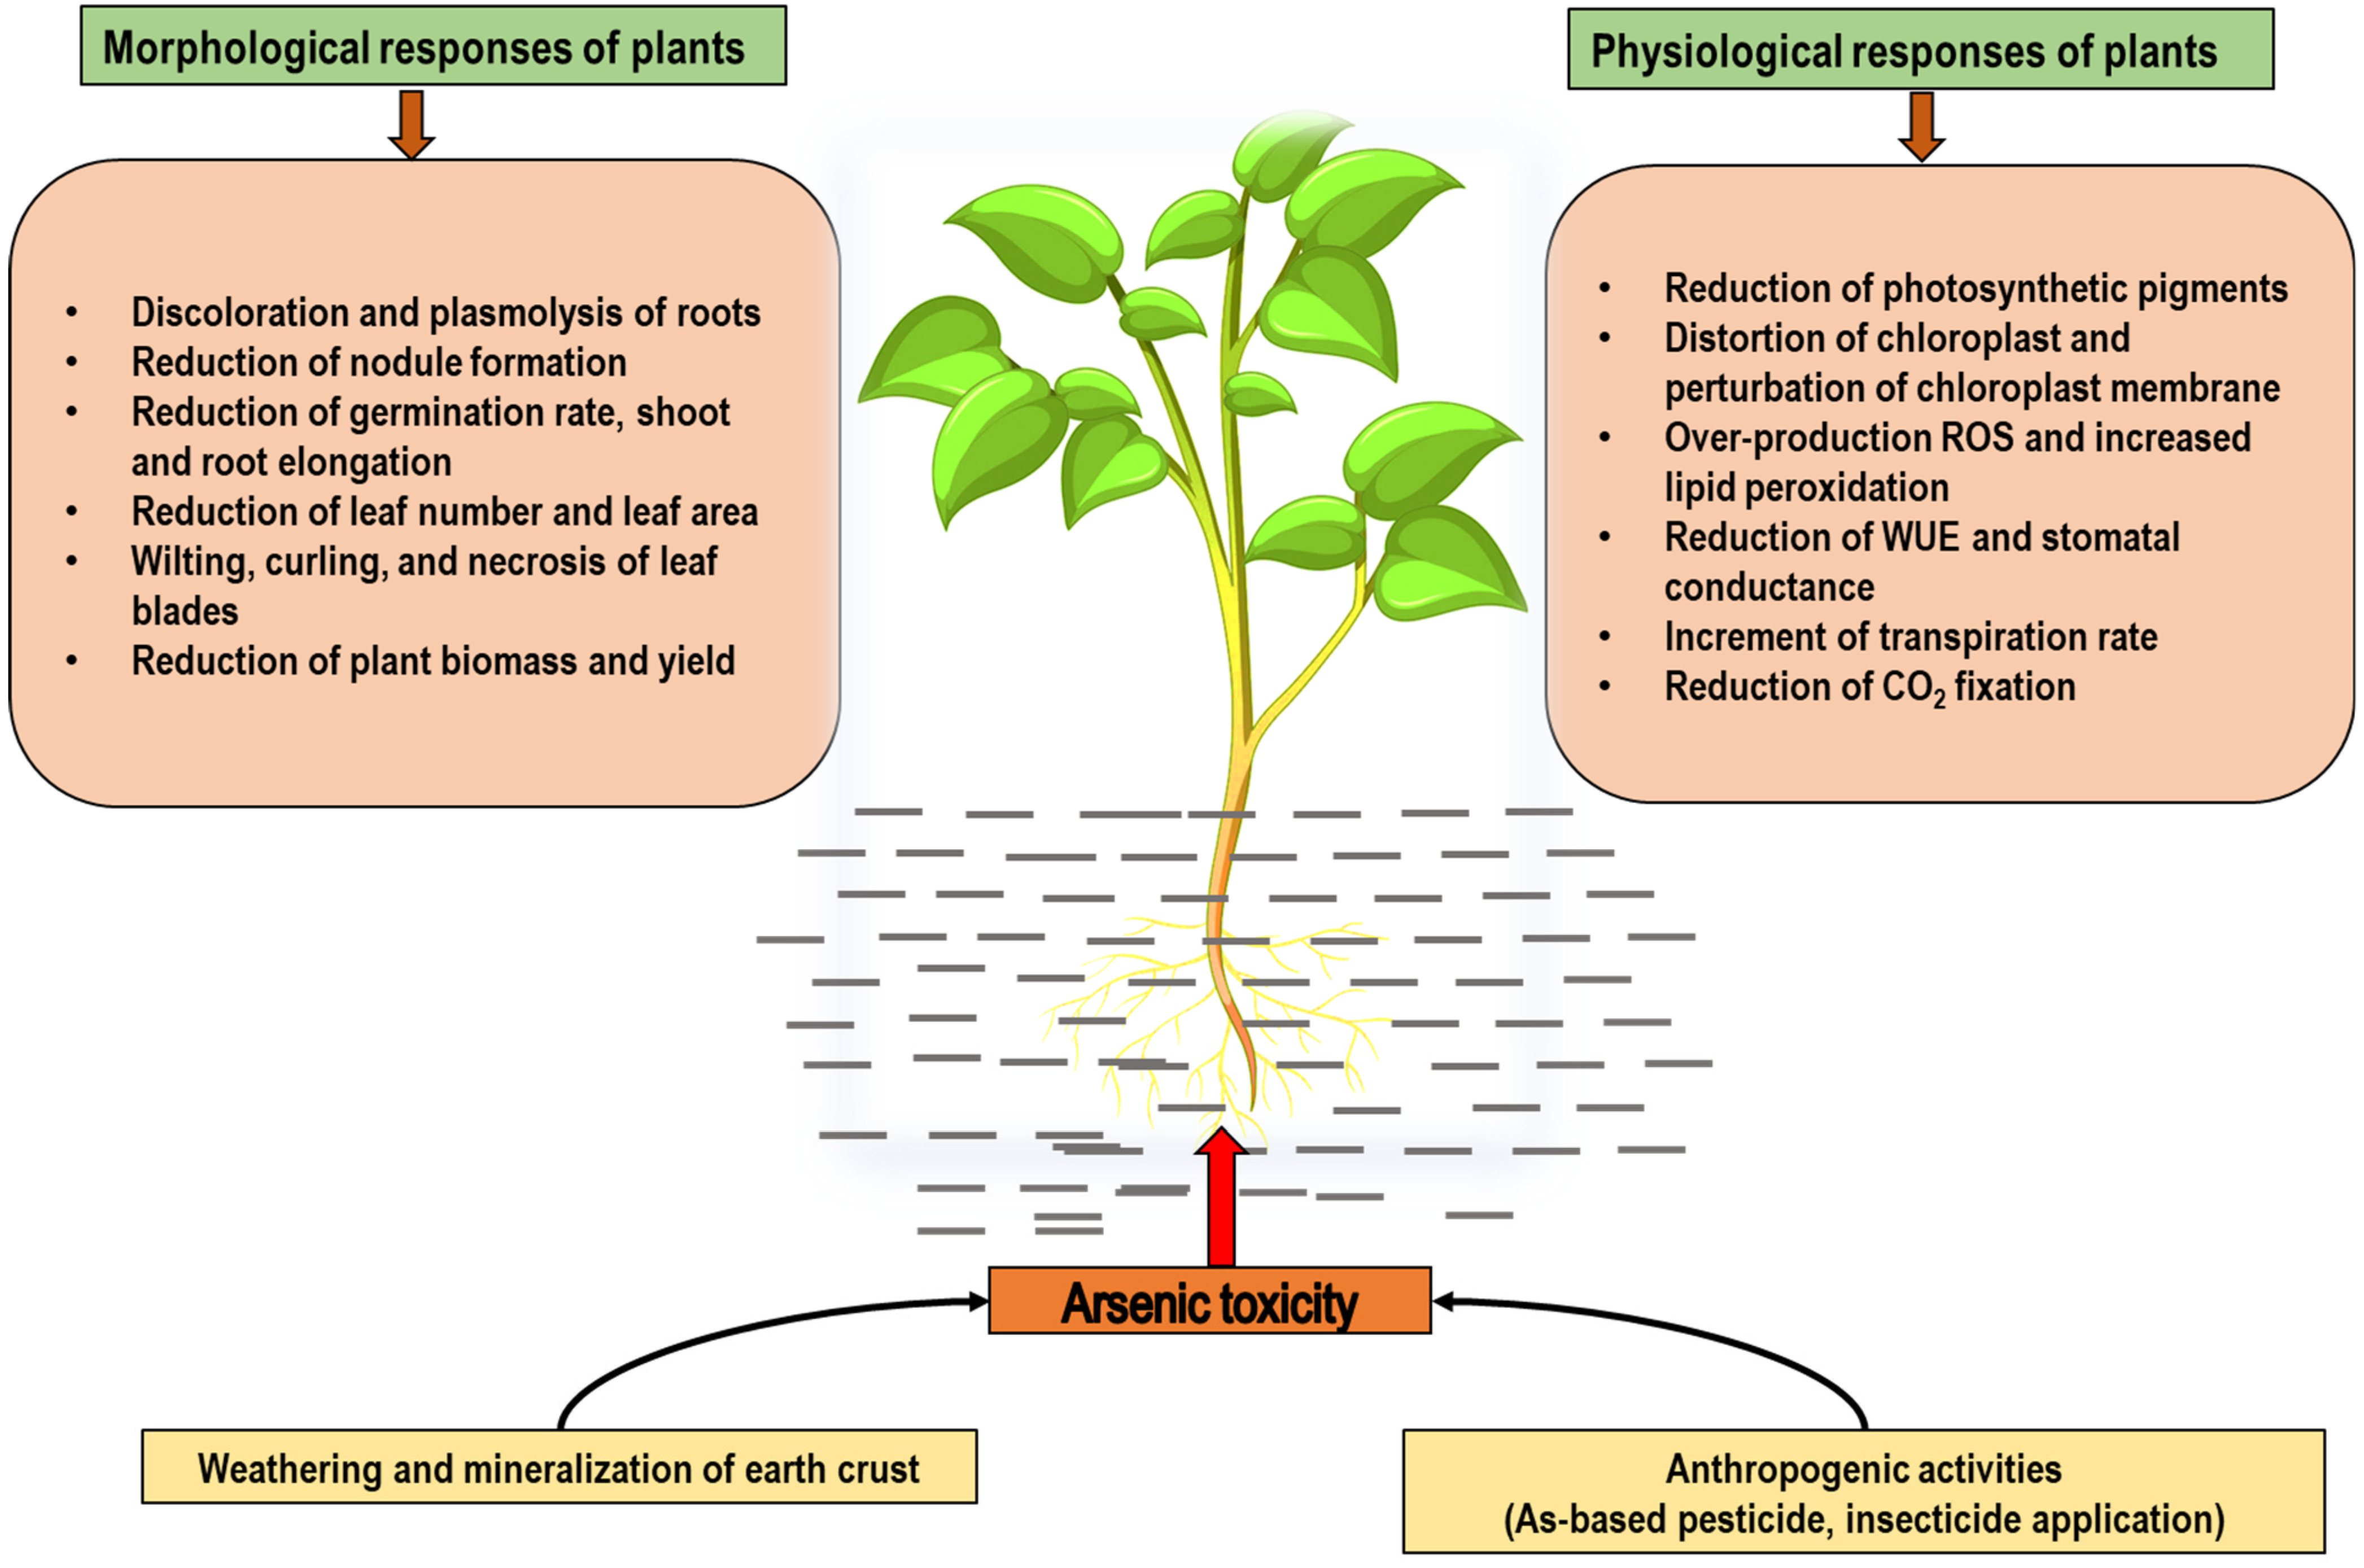
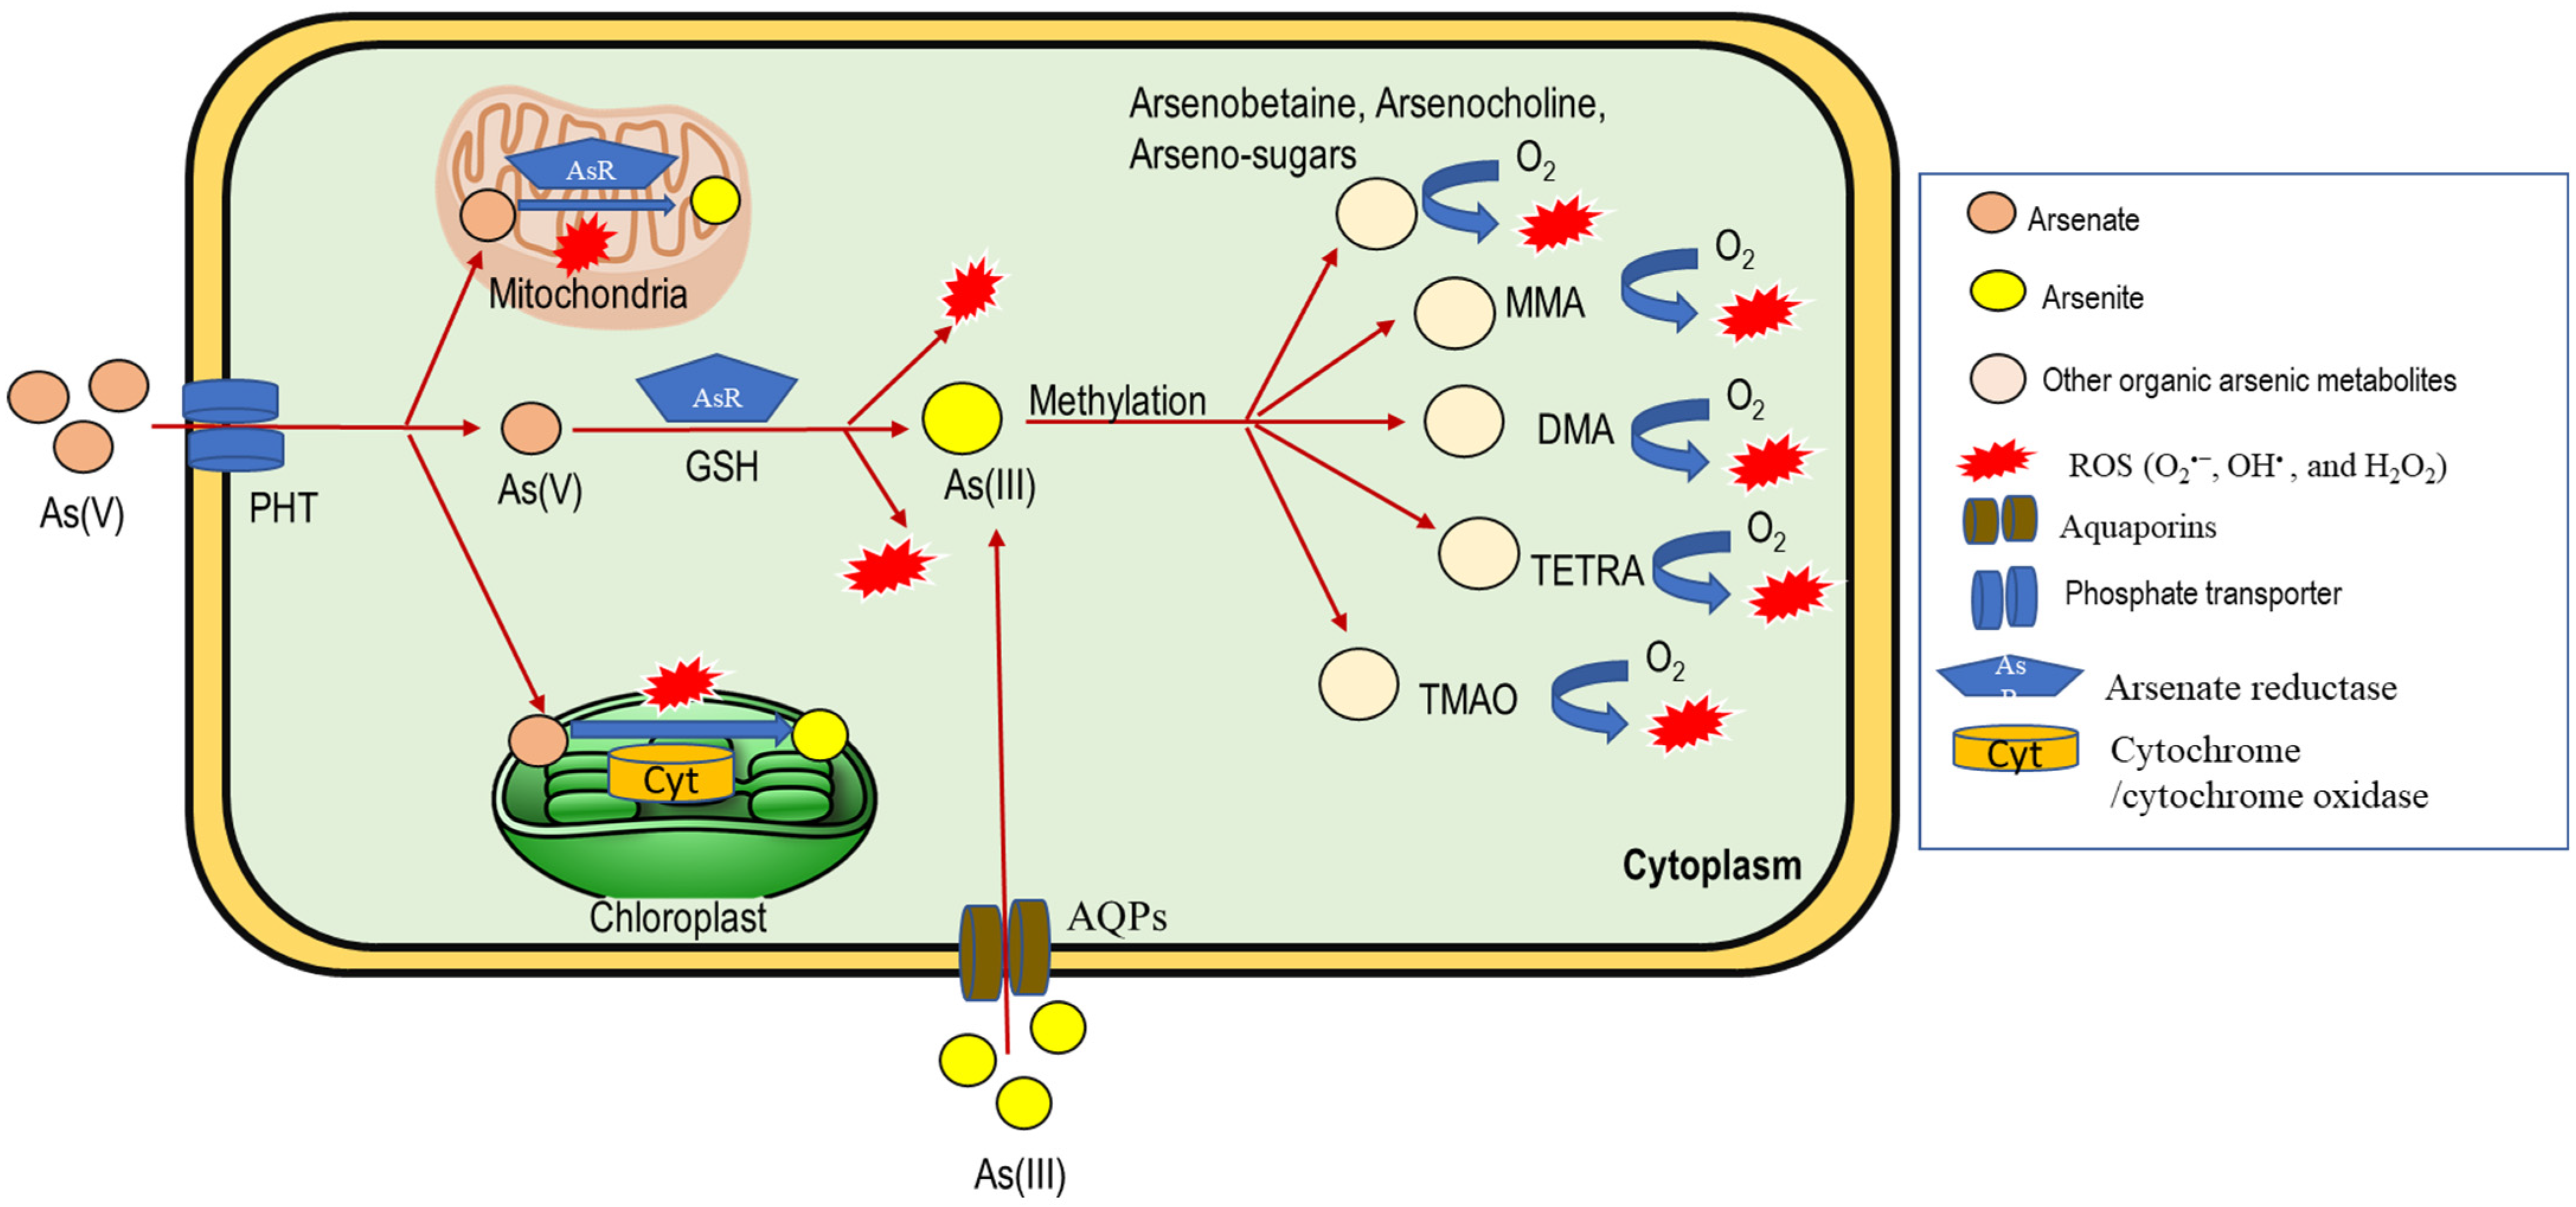
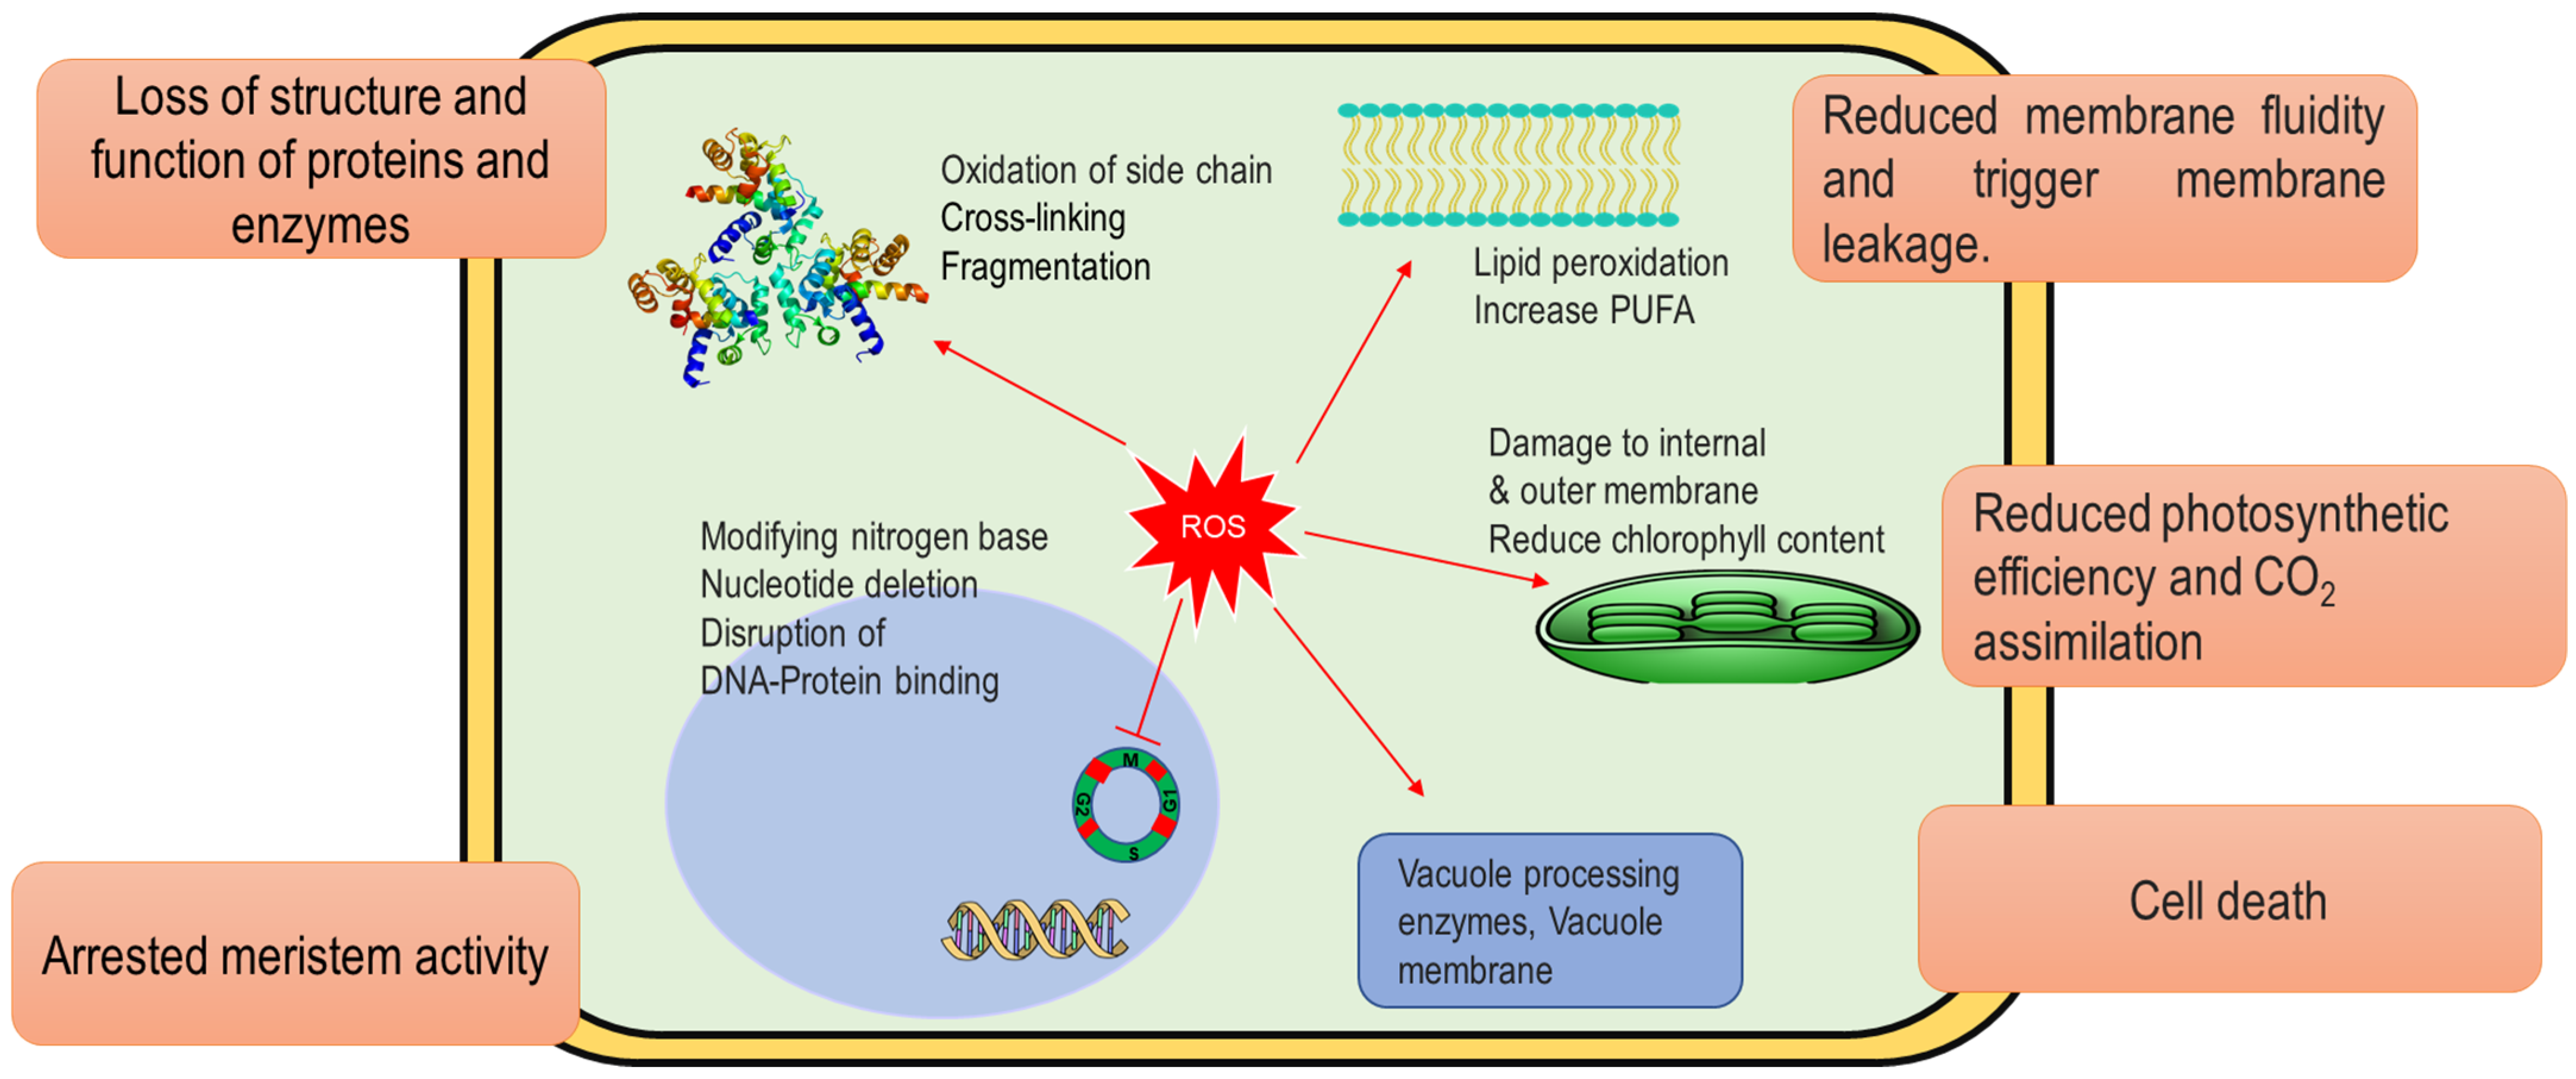

Publisher’s Note: MDPI stays neutral with regard to jurisdictional claims in published maps and institutional affiliations. |
© 2022 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).