


Simple Summary
Many forest animals are difficult to monitor because they are rare, elusive, or active at night. Camera traps provide a non-invasive way to observe these species, but short surveys may fail to capture the full wildlife community. We used ten years of camera-trap records from the Baishuihe National Nature Reserve in southwestern China to examine how the understanding of a mountain wildlife community changes with continued monitoring. As monitoring progressed, fewer previously undetected species were added, while the species most frequently recorded remained consistently present. Wildlife species also differed in the times of day when they were active, which may help them reduce encounters and share habitats and resources. These findings show that long-term camera-trap monitoring is important for distinguishing persistent ecological patterns from short-term variation in wildlife records. The study provides baseline information that can support biodiversity monitoring and conservation management in the Giant Panda National Park and other mountain protected areas in southwestern China.
Abstract
Long-term ecological monitoring is essential for understanding biodiversity dynamics and evaluating conservation effectiveness in protected areas. The Baishuihe National Nature Reserve, located in the southern Minshan Mountains, represents an important montane forest ecosystem within a global biodiversity hotspot. Using camera-trapping data collected from 2011 to 2020, we investigated long-term community dynamics and temporal activity patterns of mammals and ground-dwelling pheasants in the reserve. A total of 23 species, including 17 mammal and 6 pheasant species, were recorded during the 10-year survey. Carnivora and Artiodactyla were the most species-rich orders, while several ungulates and pheasants dominated detections throughout the monitoring period. Species richness increased with survey duration, while the rate of newly recorded species declined after 2016, and the observed assemblage became more consistent across years. Interannual community variation reflected both species turnover and nestedness-related processes, although dominant and common species remained consistently detected across years. Camera-trap data further revealed pronounced temporal niche differentiation among sympatric species. Carnivores, such as leopard cat (Prionailurus bengalensis) and masked palm civet (Paguma larvata), were primarily nocturnal, whereas golden snub-nosed monkey (Rhinopithecus roxellana), Temminck’s tragopan (Tragopan temminckii), and blood pheasant (Ithaginis cruentus) showed predominantly diurnal activity patterns. Several species exhibited broad temporal niches or seasonal shifts in activity rhythms, suggesting flexible behavioral adaptation to environmental conditions. Overall, the Baishuihe Reserve supported a taxonomically and functionally diverse camera-trap-detectable vertebrate assemblage, within which dominant and common species showed relatively persistent occurrence across years. This study highlights the importance of long-term camera-trap monitoring for understanding community stability, temporal niche organization, and biodiversity conservation in mountain ecosystems.
1. Introduction
Biodiversity is declining globally as a result of habitat loss, fragmentation, overexploitation, and other anthropogenic pressures, leading to widespread changes in species distributions and ecosystem functioning [1,2]. Protected areas are widely recognized as one of the most effective strategies for conserving biodiversity and maintaining ecosystem integrity [3,4,5,6]. However, increasing human disturbance and environmental change continue to threaten many protected ecosystems, highlighting the need for long-term ecological monitoring to evaluate conservation effectiveness and ecosystem stability over time [7,8]. Mammals and other high-trophic-level vertebrates are particularly useful indicators of ecosystem condition because their community composition, population persistence, and behavioral dynamics often respond sensitively to environmental change [9,10].
Understanding long-term community dynamics is therefore important for assessing biodiversity conservation within protected areas [7,11,12]. In addition to changes in species composition, temporal activity patterns provide important insights into ecological interactions and coexistence mechanisms among sympatric species. Temporal niche differentiation can reduce interspecific competition and promote community stability, particularly in species-rich montane ecosystems where multiple taxa share similar habitats and resources [13,14,15]. Seasonal or interannual shifts in activity rhythms may further reflect behavioral adaptation to environmental variation and anthropogenic disturbance [16,17,18]. Consequently, analyses integrating community dynamics and activity patterns can improve our understanding of ecosystem stability and species coexistence in protected mountain ecosystems.
Because many mammal species are cryptic, elusive, and primarily nocturnal, traditional survey methods are often insufficient for continuous and long-term monitoring. Camera trapping has become one of the most widely used approaches in wildlife ecology because it enables non-invasive, continuous, and standardized monitoring of wildlife communities over extended periods [19,20]. Long-term camera-trap datasets can simultaneously provide information on species occurrence, community composition, and temporal activity patterns, making them particularly valuable for investigating wildlife community dynamics in protected areas.
The Mountains of Southwest China constitute one of the world’s biodiversity hotspots [21]. Characterized by complex topography, steep elevational gradients, and diverse climatic conditions, this region supports highly heterogeneous montane ecosystems and exceptionally rich vertebrate diversity. It also provides critical habitat for numerous rare and endangered species, including the giant panda (Ailuropoda melanoleuca), golden snub-nosed monkey (Rhinopithecus roxellana), and takin (Budorcas tibetana). Because montane ecosystems are highly sensitive to climate change and human disturbances, long-term wildlife monitoring is essential for understanding changes in community structure and ecosystem functioning in this region.
The Sichuan Baishuihe National Nature Reserve, located in the southern Minshan Mountains on the western edge of the Sichuan Basin, was established primarily to conserve giant pandas, forest ecosystems, and regional biodiversity. The reserve represents an important ecological transition zone between the Chengdu Plain and the mountainous regions of western Sichuan and contains typical montane forest ecosystems. A comprehensive biodiversity survey conducted in 2010 documented 96 mammal species and 280 bird species within the reserve, indicating high vertebrate biodiversity. However, previous studies in this region have mainly focused on flagship species or single taxonomic groups, whereas long-term community-level studies remain limited. In particular, interannual community dynamics and temporal niche organization of mammals and ground-dwelling pheasants within the reserve remain poorly understood. Moreover, earlier camera-trap studies were generally based on relatively limited spatial coverage and short monitoring durations, potentially constraining understanding of long-term ecological dynamics within the reserve.
In this study, we analyzed camera-trap data collected from more than 200 camera-trap stations in the Sichuan Baishuihe National Nature Reserve between 2011 and 2020 to investigate long-term community dynamics and temporal activity patterns of mammals and ground-dwelling pheasants. Specifically, we aimed to: (1) characterize community composition and evaluate long-term community stability; (2) describe interannual changes in the observed species inventory; and (3) examine temporal activity patterns and niche differentiation among the recorded species, with detailed comparisons focusing on species with sufficient detection records. Our study provides baseline data for long-term biodiversity monitoring and contributes to understanding community stability and wildlife conservation in montane ecosystems in the Mountains of Southwest China.
2. Materials and Methods
2.1. Study Area
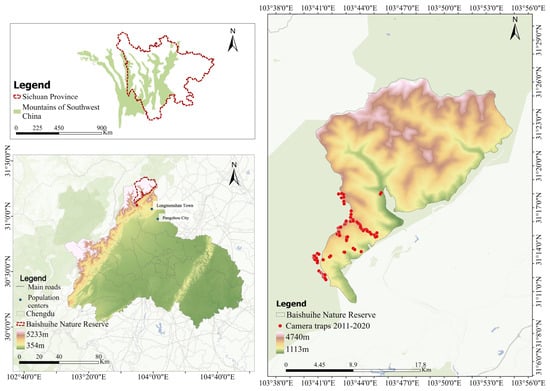
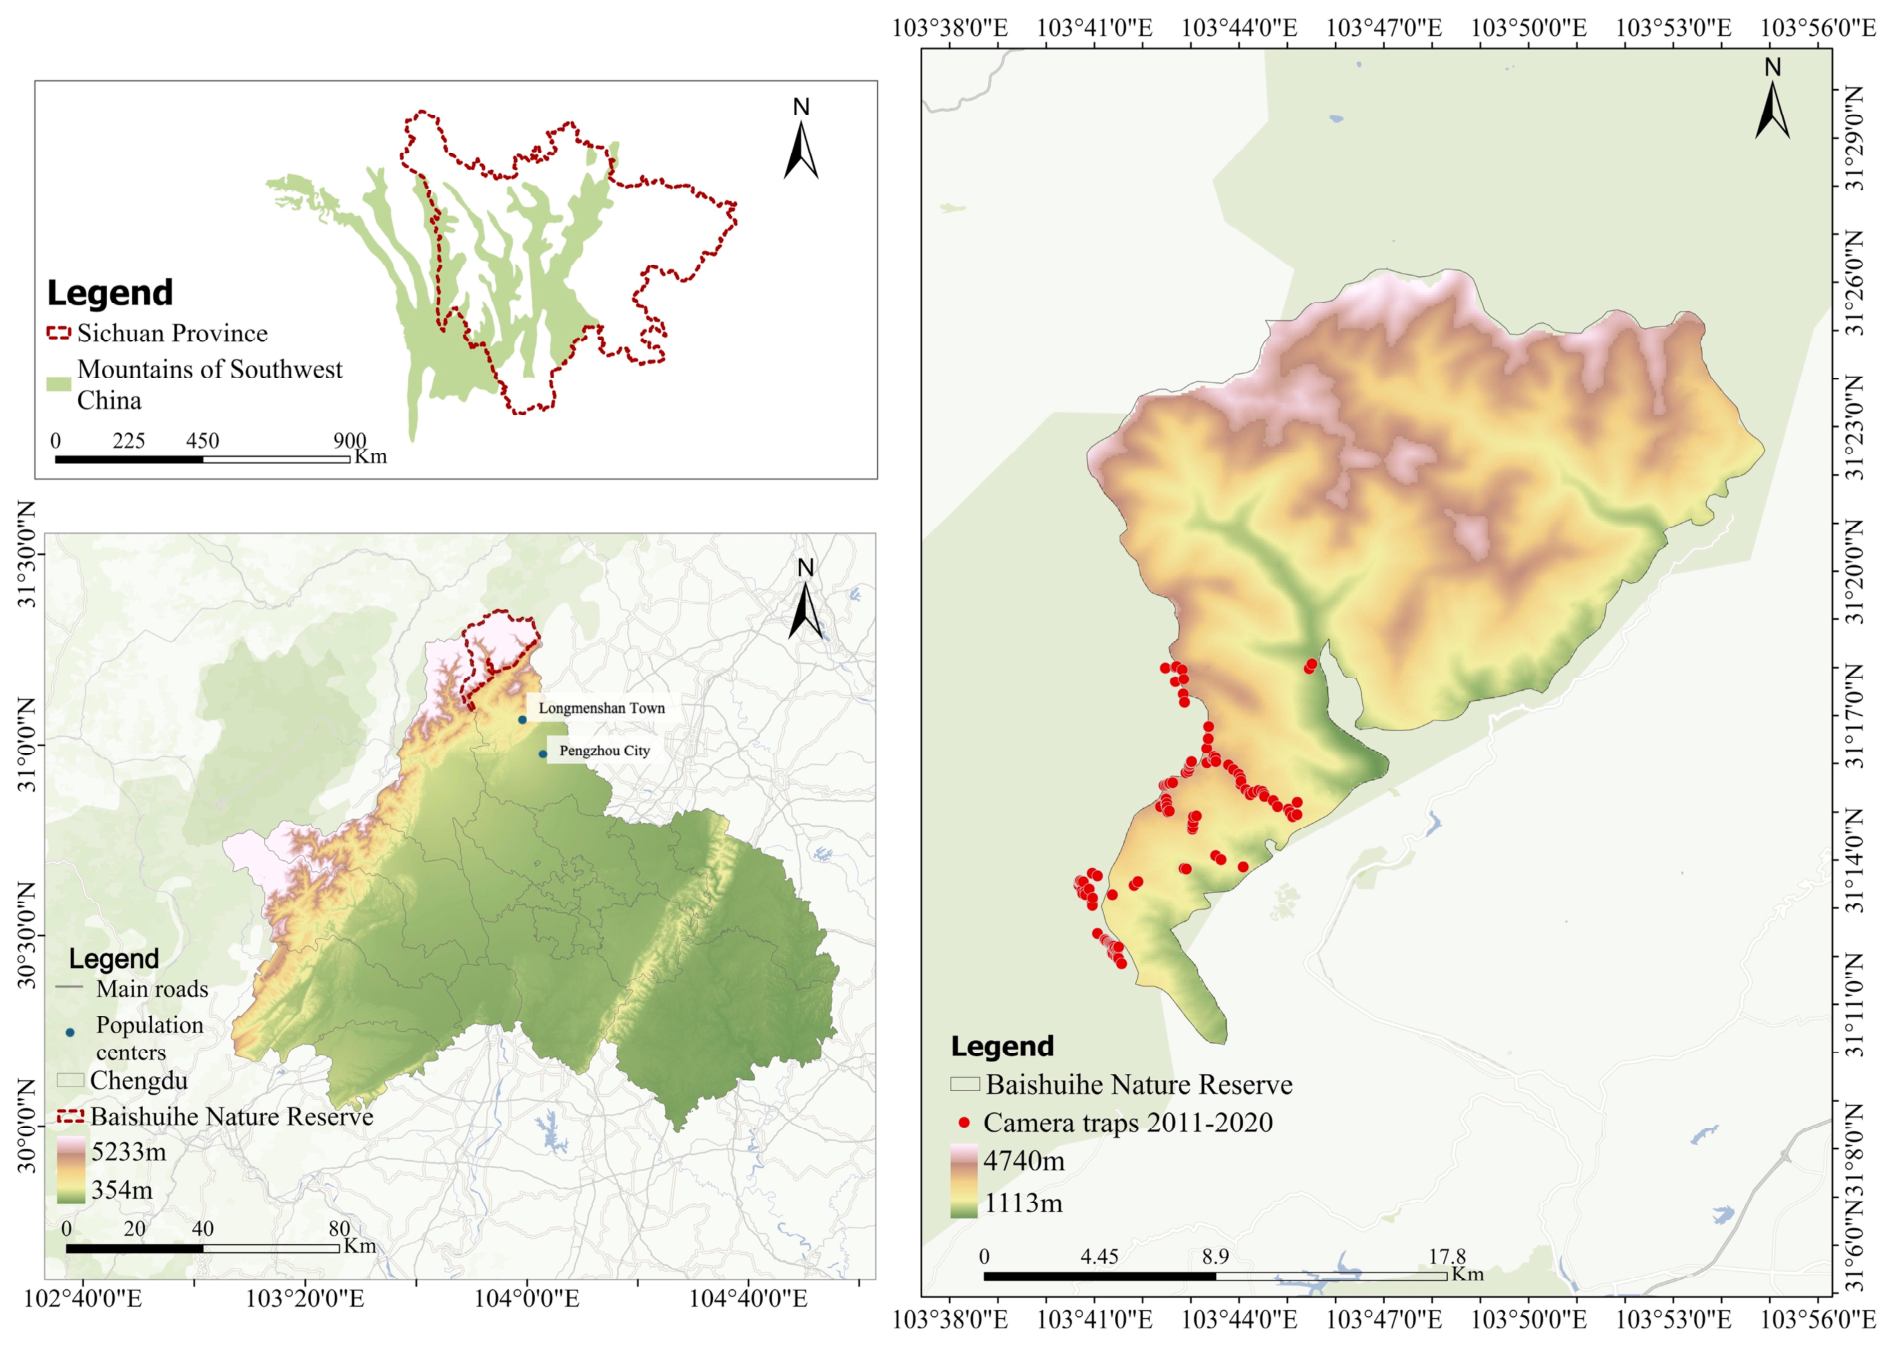
The Baishuihe Reserve (103°41′–103°57′ E, 31°10′–31°29′ N) is located in Pengzhou City, Sichuan Province, southwestern China (Figure 1). Situated in the southeastern Longmen Mountains, the reserve lies within the transitional zone between the Sichuan Basin and the Qinghai–Tibet Plateau and represents a typical montane ecotone. The reserve covers approximately 301.5 km2 and was established primarily to protect the giant panda, its habitat, rare wildlife resources, and regional biodiversity. Elevation ranges from 1481 to 4814 m above sea level, creating pronounced topographic and climatic gradients. Well-preserved montane valleys, river systems, and forest ecosystems provide diverse habitats for wildlife species.
Figure 1.
Geographic location of the Baishuihe National Nature Reserve and camera-trap stations. The upper-left panel shows the Mountains of Southwest China; the lower-left panel shows Chengdu City, major population centers, and the main road network; and the right panel shows the location, topography, and camera-trap stations of the Baishuihe National Nature Reserve during 2011–2020. The reserve is administratively located in Chengdu City and biogeographically situated within the Mountains of Southwest China.
The reserve is dominated by montane valley landforms and has a humid subtropical monsoon climate. Mean annual temperature is approximately 12.3 °C, with temperatures decreasing markedly from the warmer low-elevation valleys to the cold, snow-prone high-elevation zones. Mean annual precipitation is approximately 966.9 mm. Vegetation types include evergreen broad-leaved forests, mixed coniferous–broadleaf forests, subalpine coniferous forests, and shrub meadows. The combination of complex terrain, strong elevational gradients, and heterogeneous vegetation contributes substantially to regional biodiversity. In addition, the reserve is located between the Jiudingshan Provincial Nature Reserve and the Longxi–Hongkou National Nature Reserve, serving as an important ecological corridor and habitat connectivity zone for giant pandas in the Longmen Mountain region. Therefore, it plays a significant role in regional ecological security and wildlife dispersal.
2.2. Data Collection
Camera-Trap Survey
To monitor long-term dynamics of mammal communities in the study area, camera traps were continuously deployed throughout the reserve from 2011 to 2020. Cameras were primarily installed in areas with frequent wildlife activity, including animal trails, water sources, forest paths, and feeding sites, in order to maximize detection probability of target species [22]. Camera placement also considered elevational gradients and habitat heterogeneity to ensure broad coverage of major habitat types within the reserve.
Camera traps were generally mounted 40–60 cm above the ground, and camera lenses were positioned perpendicular to the expected direction of animal movement to reduce missed detections and false triggers. All cameras operated continuously for 24 h per day. Batteries and memory cards were checked and replaced regularly to ensure continuous operation and data integrity [23].
Following standard camera-trap survey protocols [20], consecutive photographs or videos of the same species captured at the same camera station within a 30 min interval were treated as one independent detection event to minimize repeated records of the same individual. Records of a different species, records from a different camera station, or records of the same species separated by more than 30 min were treated as separate independent events. Recorded information included capture time, species identity, number of independent detections, and activity period [24]. A single camera operating continuously for 24 h was defined as one camera day, and the effective number of camera days for each station was calculated from the interval between the first and last valid records obtained by that camera [25]. Records falling outside the predefined study period of 2011–2020 were excluded before the calculation of sampling effort. The final dataset contained 47,137 time-stamped records from 251 camera-trap stations, representing a cumulative sampling effort of 55,080.9 camera-trap days, rounded to 55,081 camera-trap days.
To evaluate relative activity intensity among species, we calculated the Relative Abundance Index (RAI). The RAI has been widely used in camera-trap studies as an indicator of relative population size and activity intensity [20,26]. The index was calculated as follows:
where the number of independent detection events represents the total number of independent records for a given species, and total camera-trap days represents the cumulative number of effective camera-trap days during the survey.
RAI = (independent detection events/total camera-trap days) × 1000
2.3. Data Analysis
2.3.1. Community Composition Analysis
Based on the camera-trap monitoring data, all recorded mammal and pheasant species were identified and compiled to establish a species inventory for the study area. Total species richness and annual species richness were calculated to characterize temporal variation in community composition. In addition, species were classified according to their taxonomic groups (order and family) to describe the taxonomic structure of the animal community.
The Relative Abundance Index (RAI) of each species was calculated from the number of independent detections and used as an indicator of relative activity intensity and relative abundance. Species accounting for more than 5% of the total independent detections were defined as dominant species and were used to identify major community components and core taxa within the study area. Species were further ranked according to their RAI values to examine patterns among dominant and infrequently detected species.
Furthermore, based on ecological functional traits, the trophic structure of the animal community was categorized into several functional groups, including carnivores, ungulates, primates, and ground-dwelling pheasants, in order to evaluate community structural integrity and ecological functional composition.
2.3.2. Interannual Dynamics Analysis
To investigate long-term community dynamics, species composition and detection records were compared among years from 2011 to 2020. Annual species richness and the number of newly recorded species in each year were summarized to describe changes in the observed species inventory over time. We used these descriptive temporal summaries to evaluate whether the addition of previously unrecorded species declined during the later monitoring period. Formal species accumulation or rarefaction curves were not generated because camera-trap effort, spatial coverage, and station numbers varied among years.
Species occurrence patterns among years were compared descriptively by summarizing newly recorded species, repeatedly recorded species, and species that were not detected in subsequent years. Interannual changes in the observed species inventory were interpreted qualitatively in relation to species addition, replacement, and nestedness-like patterns. Formal β-diversity decomposition into turnover and nestedness components was not conducted because annual sampling effort, camera-station numbers, and spatial coverage were not fully standardized across years [27].
In addition, several dominant species with relatively high detection frequencies, including Chinese goral (Naemorhedus griseus), Temminck’s tragopan (Tragopan temminckii), blood pheasant, tufted deer (Elaphodus cephalophus), and Siberian weasel (Mustela sibirica), were selected for interannual comparisons of independent detections and RAI values to evaluate temporal variation in activity intensity. Because camera numbers, monitoring duration, and effective camera days varied among years, RAI values were primarily used to reflect relative activity variation rather than absolute population size estimates [19].
To further evaluate the effectiveness of long-term monitoring, the number of newly recorded species was also summarized for each year, and temporal trends in species accumulation were examined to assess whether community composition approached stability over time. A marked decline in newly recorded species during later monitoring periods was considered indicative of sufficient sampling coverage of the camera-trap-detectable mammal and ground-dwelling pheasant assemblages in the reserve [28].
2.3.3. Activity Pattern Analysis
Activity patterns of the recorded mammal and pheasant species were analyzed based on the timestamps recorded by camera traps. Following established approaches in camera-trap activity studies [29,30], the exact detection time of each independent event was extracted, and temporal activity distributions of different species were summarized over a 24 h cycle.
Based on local daylight conditions and previous studies, the 24 h period was divided into daytime (06:00–18:00) and nighttime (18:00–06:00), while crepuscular activity periods were also considered in activity classification. According to the proportion of independent detections distributed across different time periods, species were classified into four activity categories: (1) diurnal, with activity concentrated mainly during daytime; (2) nocturnal, with activity concentrated mainly during nighttime; (3) cathemeral, with relatively high activity frequencies during both day and night and no clear diel preference; and (4) seasonally variable, with marked seasonal shifts in activity time distribution.
For species with relatively large sample sizes, monthly and seasonal variation in activity time distributions were further examined to evaluate seasonal changes in activity rhythms. In particular, seasonal variation in the proportion of daytime and nighttime detections was compared to explore potential influences of environmental conditions on species activity strategies. Previous studies have demonstrated that animal activity rhythms can be affected by multiple factors, including temperature, food resource availability, anthropogenic disturbance, and predation risk [31,32].
In addition, activity patterns were compared among different functional groups, including carnivores, ungulates, primates, and ground-dwelling pheasants, to examine differences in temporal resource use among trophic groups. Based on temporal overlap in activity among species, temporal niche partitioning within the animal community was qualitatively evaluated, and potential mechanisms by which species reduce resource competition and interference through temporal segregation were discussed [33].
Because sample sizes for some species were limited, activity pattern analyses in this study were primarily descriptive and qualitative. Quantitative analyses, such as those of activity overlap indices and kernel density estimation, were not conducted. Nevertheless, the results provide useful descriptive insights into the activity patterns and temporal niche differentiation of the recorded species, particularly those with sufficient detection records.
3. Results
3.1. Community Composition
The survey recorded 17 mammal species and 6 pheasant species, comprising 23 species in total. Mammals belonged to 4 orders and 10 families, whereas all recorded bird species belonged to the order Galliformes and the family Phasianidae. The recorded fauna included carnivores, medium- and large-sized ungulates, primates, and ground-dwelling pheasants, representing multiple ecological functional groups.
Among mammals, Carnivora was the most species-rich order, comprising 8 species from 4 families: giant panda (Ailuropoda melanoleuca), Asian black bear (Ursus thibetanus), yellow-throated marten (Martes flavigula), Siberian weasel (Mustela sibirica), hog badger (Arctonyx collaris), Asian badger (Meles leucurus), masked palm civet (Paguma larvata), and leopard cat (Prionailurus bengalensis), accounting for 47.1% of the recorded mammal species. Artiodactyla was the second most species-rich order, comprising 6 species from 4 families: tufted deer (Elaphodus cephalophus), Chinese serow (Capricornis milneedwardsii), Chinese goral (Naemorhedus griseus), takin (Budorcas tibetanus), wild boar (Sus scrofa), and forest musk deer (Moschus berezovskii), accounting for 35.3% of the recorded mammal species. In addition, two primate species, Tibetan macaque (Macaca thibetana) and golden snub-nosed monkey (Rhinopithecus roxellana), and one rodent species, Chinese porcupine (Hystrix hodgsoni), were recorded. Six pheasant species were detected, including Temminck’s tragopan (Tragopan temminckii), blood pheasant (Ithaginis cruentus), Chinese monal (Lophophorus lhuysii), golden pheasant (Chrysolophus pictus), koklass pheasant (Pucrasia macrolopha), and chestnut-throated partridge (Tetraophasis obscurus) (Table 1).
Table 1.
Species composition, relative abundance index (RAI), and conservation status of mammals and pheasants recorded in the Baishuihe National Nature Reserve during 2011–2020.
Relative abundance analysis based on independent detection events revealed substantial variation in detection frequency among species. Chinese goral was the most frequently detected species, with 575 independent detections, accounting for 22.2% of all records. This was followed by Temminck’s tragopan (387 detections, 15.0%) and blood pheasant (272 detections, 10.5%). Tufted deer (205 detections, 7.9%), Siberian weasel (181 detections, 7.0%), and Tibetan macaque (149 detections, 5.8%) also exhibited relatively high detection frequencies. These six species all accounted for more than 5% of total detections and were therefore identified as dominant species. Together, they represented 68.4% of all independent detections, indicating a community structure characterized by a clear concentration of dominant species.
In addition to dominant species, takin (111 detections, 4.3%) and yellow-throated marten (110 detections, 4.3%) were also frequently recorded and could be considered common species in the monitored area. In contrast, giant panda (4 detections) and koklass pheasant (2 detections) were rarely detected and occurred only at a few camera stations or during specific years. These records indicate low detection frequencies in the present camera-trap dataset, but they should not be interpreted directly as evidence of low local abundance, particularly across the entire reserve. For giant panda, the low number of detections may partly reflect the fact that the camera-trap survey covered only part of the reserve and may not have fully overlapped with the main areas of giant panda habitat use. More generally, low detection frequencies may also result from low detection probability, behavior that reduces exposure to camera traps, restricted use of the sampled area, or occasional passage through monitored sites.
Several medium- and large-sized mammals previously reported in the 2010 baseline survey, including red panda (Ailurus fulgens), Asian golden cat (Catopuma temminckii), leopard (Panthera pardus), and clouded leopard (Neofelis nebulosa), were not detected by the present camera-trap network. Their non-detection may reflect the restricted spatial coverage of the survey, limited overlap between camera locations and species-specific habitats or movement routes, low detection probability, or very low current population densities. However, because some historical records were based on indirect survey methods and several of these species have not been confirmed in recent regional surveys, their current occurrence in the reserve remains uncertain.
From the perspective of ecological functional composition, the study area supported multiple trophic groups, including mesocarnivores, such as leopard cat and yellow-throated marten; medium- and large-sized herbivores, such as Chinese goral, tufted deer, and takin; and various pheasant and primate species. The occurrence of taxa from different trophic groups indicates that multiple trophic components were represented in the camera-trap records. However, because trophic interactions were not directly measured and no reference food web was available, these records alone cannot demonstrate the completeness or intactness of the food web. The repeated detection of carnivores and medium-to-large ungulates nevertheless suggests that the reserve continues to provide habitat for species occupying different trophic positions [34].
3.2. Interannual Dynamics
Annual sampling effort varied substantially during the monitoring period (Table 2). Annual camera-trap effort increased from 918.0 camera-trap days in 2011 to 12,509.3 camera-trap days in 2019 and then declined to 7508.9 camera-trap days in 2020. Consequently, interannual comparisons of species richness and detection frequency should be interpreted with caution because annual camera-trap effort, the number of active camera stations, and spatial coverage were not fully standardized across years.
Table 2.
Annual numbers of active camera-trap stations and sampling effort in the Baishuihe National Nature Reserve during 2011–2020. Active stations were defined as stations that yielded at least one valid time-stamped record in a given year.
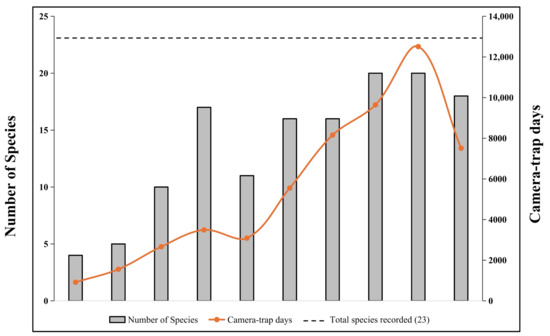
During the monitoring period, annual species richness generally increased as monitoring effort expanded. Four species were detected in 2011 and five in 2012; richness increased to 10 species in 2013 and 17 in 2014. Although richness declined to 11 species in 2015, it increased again to approximately 16 species in 2016–2017, reached 20 species in 2018–2019, and remained relatively high at 18 species in 2020. The pattern should be interpreted as variation in the observed species inventory under unequal annual sampling effort rather than direct evidence of ecological expansion of the underlying community (Figure 2).
Figure 2.
Annual species richness and camera-trap days in the Baishuihe National Nature Reserve during 2011–2020. Bars represent annual species richness, the solid line represents camera-trap days, and the dashed line indicates the 23 species recorded across the full monitoring period. Because annual station numbers and spatial coverage varied, this descriptive figure should not be interpreted as a standardized species accumulation or rarefaction curve.
Community composition varied among years. During the early monitoring period (2011–2012), relatively few species were detected, and the observed assemblage mainly consisted of common species with relatively high detection frequencies, such as tufted deer, Temminck’s tragopan, and yellow-throated marten. After 2013, species such as Chinese goral, takin, leopard cat, hog badger, and Chinese serow were detected more consistently, resulting in a progressively richer observed assemblage. Since 2014, several medium- and large-sized mammals and carnivores were repeatedly detected across multiple years, suggesting that increased monitoring effort and broader coverage improved characterization of the camera-trap-detectable assemblage.
With regard to interannual variation in dominant species, most dominant species were consistently recorded across years, indicating relatively high temporal stability. Chinese goral, Temminck’s tragopan, and blood pheasant maintained relatively high detection frequencies throughout most years and represented the most stable core species within the study area. Tufted deer and Siberian weasel were also recorded in all years, although their detection frequencies fluctuated more substantially. In contrast, several low-frequency species occurred only sporadically. For example, koklass pheasant and chestnut-throated partridge were detected infrequently, and their occurrences among years appeared highly stochastic.
From the perspective of community dynamics, changes in the animal community were primarily characterized by a gradual increase in newly recorded species. The period from 2013 to 2014 represented the most pronounced stage of species increase, during which several medium- and large-sized mammals and carnivores were first detected. After 2016, the number of newly recorded species declined markedly, and the observed annual assemblage became more consistent relative to the early monitoring period of 2011–2015. Here, this increased consistency refers to a lower rate of species addition and the repeated detection of dominant and common species. Overall, the observed species inventory showed both the addition or replacement of some species among years and nestedness-like variation, in which species-poor years largely represented subsets of species-rich years. However, because no formal β-diversity decomposition was conducted, this interpretation should be regarded as descriptive rather than quantitative. Specifically, some community changes reflected gradual detection of previously unrecorded species, whereas fluctuations in low-frequency species contributed to nestedness-related patterns.
In addition, the core community composition gradually stabilized with increasing monitoring duration. Most dominant and common species were consistently recorded across consecutive years, while the number of newly detected species progressively declined, indicating relatively high long-term stability of mammal and ground-dwelling bird communities in the reserve. Overall, long-term camera-trap monitoring not only improved the detection of regional biodiversity but also revealed the dynamic process through which the animal community transitioned from an initial low-detection stage to a relatively stable state over time.
3.3. Activity Patterns
Based on the timestamps recorded by camera traps, activity time distributions of the 23 recorded species were summarized and analyzed. The results showed clear diel activity differentiation within the animal community, with substantial variation in activity timing among species. According to the distribution of independent detections across daytime and nighttime periods, species activity patterns could be classified into four categories: typical diurnal, typical nocturnal, cathemeral, and seasonally variable activity patterns [35] (Figure 3).
Figure 3.
Daily activity patterns of six dominant mammal and pheasant species in the Baishuihe National Nature Reserve: Elaphodus cephalophus, Ithaginis cruentus, Tragopan temminckii, Naemorhedus griseus, Macaca thibetana and Mustela sibirica.
- (1)
- Typical Diurnal Species
Diurnal species were characterized by activity concentrated mainly during daytime hours (approximately 06:00–18:30), with few or no nighttime records. All detections of golden snub-nosed monkey and Chinese monal occurred during daytime, indicating strongly diurnal activity patterns. Asian black bear, wild boar, yellow-throated marten, Temminck’s tragopan, and blood pheasant were also primarily active during daytime, with only occasional nighttime detections.
Among these species, Temminck’s tragopan and blood pheasant showed peak activity primarily during the early morning to late morning period (approximately 07:00–11:00), after which activity frequency declined in the afternoon. Yellow-throated marten exhibited relatively high activity frequencies throughout multiple daytime periods, indicating a relatively broad diurnal activity range. Overall, diurnal species were mainly associated with visually oriented foraging behavior or group activities, and their activity schedules appeared closely related to daylight availability and feeding behavior.
- (2)
- Typical Nocturnal Species
Nocturnal species were primarily active during nighttime and early morning hours (approximately 18:00–06:00), with relatively few daytime records. Leopard cat, masked palm civet, and Chinese porcupine all exhibited clear nocturnal activity patterns, with activity peaks occurring mainly during nighttime and pre-dawn periods. Leopard cat activity was concentrated primarily after 20:00, whereas Chinese porcupine showed particularly high activity frequencies during late-night to early-morning hours.
Forest musk deer also displayed predominantly nocturnal behavior in most monitoring years, with nighttime detections occurring much more frequently than daytime records. Hog badger and Asian badger similarly exhibited nocturnal tendencies, with only occasional daytime detections. Although tufted deer were detected throughout the 24 h cycle, activity was more concentrated during nighttime and crepuscular periods, particularly shortly after sunset and before sunrise, indicating an overall tendency toward nocturnal activity.
Overall, nocturnal species were mainly composed of cryptic small- and medium-sized mammals. Their nocturnal activity patterns may be associated with avoidance of anthropogenic disturbance, reduction in predation risk, and nocturnal foraging strategies.
- (3)
- Cathemeral Species
Some species exhibited relatively high activity frequencies during both daytime and nighttime and showed no obvious diel preference and were therefore classified as cathemeral species. Siberian weasel and Chinese goral consistently exhibited typical cathemeral activity patterns throughout all monitoring years, with independent detections relatively evenly distributed across day and night periods. Takin showed similar activity patterns in most years, suggesting a broad temporal activity range.
Chinese goral maintained relatively high detection frequencies during both daytime and nighttime, indicating strong environmental adaptability. Siberian weasel exhibited multiple activity peaks across both day and night periods, with relatively dispersed activity rhythms. Takin showed frequent nighttime activity while also maintaining stable daytime detections, suggesting high temporal flexibility in foraging and movement behavior.
Cathemeral species generally occupied broader temporal niches, and such activity patterns may enhance resource utilization efficiency while reducing direct temporal competition with other species.
- (4)
- Seasonally Variable Activity Patterns
Some species exhibited marked seasonal variation in activity rhythms, indicating relatively high temporal niche plasticity. Tibetan macaque was primarily active during nighttime and early morning periods in warmer months (May–October), whereas daytime activity became dominant during winter (December), demonstrating clear seasonal shifts in activity patterns.
Temminck’s tragopan exhibited a typical diurnal pattern during most months; however, nighttime and pre-dawn detections increased noticeably from October to December, indicating a tendency toward increased nocturnal activity during winter. This pattern suggests that some species may adjust their activity schedules in response to seasonal changes in temperature, food resource availability, or anthropogenic disturbance.
In addition, activity peaks of several species varied seasonally. For example, tufted deer and Chinese goral exhibited increased crepuscular activity during winter, whereas their activity distributions became more evenly distributed during summer. Overall, some species in the study area appeared capable of flexibly adjusting their activity rhythms in response to environmental variation, reflecting relatively strong ecological adaptability.
Overall, mammals and pheasants in the study area exhibited clear temporal niche partitioning. Diurnal, nocturnal, and cathemeral species coexisted within the community, resulting in temporal segregation among species and potentially reducing resource competition and interference risk. Furthermore, seasonal shifts in activity rhythms observed in several species suggest that the animal community possesses relatively high ecological adaptability and temporal resource partitioning capacity.
4. Discussion
4.1. The Baishuihe Reserve Supports a Taxonomically and Functionally Diverse Montane Vertebrate Assemblage
Long-term camera-trap monitoring recorded 17 mammal species and 6 pheasant species in the Baishuihe Nature Reserve, representing multiple trophic and functional groups, including carnivores, ungulates, primates, and pheasants. The continued occurrence of medium- and large-sized herbivores, such as Chinese goral, tufted deer, and Sichuan takin, together with mesocarnivores, including leopard cat and yellow-throated marten, suggests that the reserve maintains relatively high faunal diversity and retains key trophic components of montane forest ecosystems.
Previous studies have shown that carnivores and ungulates are highly sensitive to habitat fragmentation and human disturbance, and their persistence is often associated with relatively intact forest ecosystems and stable habitat conditions [36,37,38]. In this study, several carnivores and ungulates were consistently detected across multiple years, indicating long-term persistence of core trophic groups within the reserve. The coexistence of predators, herbivores, and primates further suggests that ecological processes and trophic interactions remain relatively stable in the study area [39].
Ground-dwelling pheasants are also widely regarded as indicators of forest ecosystem condition because they are sensitive to understory structure and habitat disturbance [40]. Species such as Temminck’s tragopan and blood pheasant were repeatedly detected throughout the monitoring period and exhibited relatively high detection frequencies, suggesting that forest understory structure and habitat quality remain suitable for forest-dependent bird species. In particular, the continued occurrence of high-elevation pheasants, such as blood pheasant and Chinese monal, indicates alpine forest habitats within the reserve remain relatively well preserved.
Overall, the continued detection of multiple taxonomic and trophic groups indicates that the Baishuihe Nature Reserve supports a diverse camera-trap-detectable montane vertebrate assemblage. These findings highlight the importance of protected areas in maintaining biodiversity and ecological stability in the montane ecosystems.
4.2. Long-Term Monitoring Revealed Community Stabilization and Cumulative Species Detection Patterns
Species richness increased substantially throughout the monitoring period, rising from four recorded species in 2011 to approximately 20 species in later years. This pattern likely reflects the cumulative effects of long-term monitoring, as extended sampling duration and broader spatial coverage gradually improved the detectability of rare, low-density, and cryptic species. Similar species accumulation dynamics have been widely reported in long-term camera-trap studies, particularly in complex montane forest ecosystems where detection probabilities are often heterogeneous among species [20,22,37].
The relatively low species richness recorded during the initial monitoring years was most likely attributable to lower sampling effort and restricted spatial coverage during establishment of the camera-trap network. As the number and spatial coverage of camera stations increased after 2013, the probability of detecting uncommon, low-density, and cryptic species also increased. Thus, much of the early increase in recorded richness probably represents improved detection rather than rapid ecological change in the underlying community. Species such as Chinese goral, Sichuan takin, leopard cat, and hog badger were detected more consistently after 2013, further indicating that short-term surveys may underestimate biodiversity in heterogeneous mountain ecosystems [26,41,42,43].
Although species composition fluctuated among years, most dominant and common species were consistently recorded throughout the monitoring period, indicating that the core community composition remained relatively stable. In particular, the Chinese goral, Temminck’s tragopan, and blood pheasant maintained high detection frequencies throughout the study period and represented the most stable core species within the reserve. This pattern, characterized by “stable core species with fluctuating rare species,” is common in montane forest ecosystems and is generally considered indicative of high community stability and ecological resilience [44,45]. Previous studies have suggested that stable core species often play important roles in ecosystem energy flow, resource utilization, and community maintenance, whereas occasional species may primarily reflect habitat heterogeneity and stochastic dispersal processes [46,47,48].
The community dynamics observed in this study also exhibited characteristics of both species turnover and nestedness-related changes. As monitoring duration increased, several previously unrecorded species were gradually and repeatedly detected in later years, indicating that long-term monitoring continuously supplemented information on regional species composition. In contrast, some low-frequency species were detected only in specific years, reflecting temporal fluctuations in community composition. Overall, species assemblages recorded in years with lower richness largely represented subsets of those recorded in years with higher richness, suggesting that community variation exhibited a certain degree of nestedness [27].
It should be noted that the assessment of species turnover and nestedness-related changes in this study was based primarily on qualitative comparisons of species occurrence among years, rather than formal β-diversity partitioning analyses. Therefore, the observed patterns mainly reflect the gradual accumulation and identification of regional species through long-term monitoring, rather than substantial ecological succession or community reorganization. Similar studies have shown that temporal community changes in long-term ecological monitoring are often jointly influenced by both real ecological processes and cumulative sampling effects [42,49].
Furthermore, after 2016, the number of newly recorded species declined substantially, while the core community composition gradually stabilized, suggesting that long-term monitoring had captured most of the camera-trap-detectable mammal and ground-dwelling pheasant species within the reserve. This pattern of “rapid increase during the early stage followed by stabilization” is consistent with species accumulation dynamics commonly observed in long-term biodiversity monitoring studies [28]. Meanwhile, the long-term persistence of most medium- and large-sized mammals and carnivores further suggests that the Baishuihe Nature Reserve maintains a relatively stable forest ecosystem structure and plays an important role in regional biodiversity conservation.
Overall, the results of this study demonstrate that long-term camera-trap monitoring can not only substantially improve species detection efficiency but also effectively reveal the dynamic changes and stability characteristics of montane forest faunal communities, thereby providing important support for evaluating protected-area ecological functions and conservation effectiveness [50,51].
In the present dataset, the rate at which previously unrecorded species were added declined after approximately six years of monitoring. However, this empirical pattern should not be interpreted as a universal minimum or optimal monitoring duration because camera-trap effort and spatial coverage varied among years, particularly during the establishment of the monitoring network. A formal sample- or coverage-based rarefaction analysis would require standardized species detection histories across comparable sampling units. Therefore, the present study cannot determine a general monitoring-duration threshold.
Similarly, the reduction in newly recorded species suggests that sampling approached an asymptote for the mammals and ground-dwelling pheasants detectable by the camera-trap design, but it does not demonstrate complete species saturation. Arboreal species, small mammals, highly cryptic species, and species occurring outside camera detection zones may remain underrepresented.
4.3. Temporal Niche Differentiation Among Recorded Species
This study found that recorded mammal and pheasant species in the Baishuihe Nature Reserve exhibited pronounced diel activity differentiation, with different species showing distinct temporal activity patterns. The coexistence of diurnal, nocturnal, and cathemeral species indicates a high degree of temporal resource partitioning within the community. Such temporal niche differentiation is considered one of the key mechanisms maintaining multispecies coexistence in complex forest ecosystems [31,52].
Temporal niche partitioning can effectively reduce resource competition and potential interference among sympatric species. By separating activity periods, species are able to share resources while minimizing direct interactions, thereby enhancing community stability [30,33]. In this study, small- and medium-sized mammals, such as leopard cat, masked palm civet, and Chinese porcupine, were primarily nocturnal, whereas golden snub-nosed monkey, Temminck’s tragopan, and blood pheasant were mainly diurnal, forming clear diel activity segregation. Such differences in activity rhythms likely reduce direct competition among species in terms of food resources, spatial use, and behavioral activities. Similar patterns of diel niche partitioning have been widely reported in Asian montane forest ecosystems and are considered important mechanisms facilitating the long-term coexistence of small mammals and ground-dwelling birds [30].
Several mesocarnivores in the study area exhibited typical nocturnal activity patterns. In particular, leopard cats and masked palm civets showed activity peaks during nighttime and pre-dawn periods, which is likely associated with their cryptic behavior and nocturnal foraging strategies. Previous studies have shown that nocturnal activity not only improves hunting efficiency for carnivores but also reduces the risk of encounters with humans [32]. In addition, nocturnal activity may decrease spatial interference with large diurnal herbivores, thereby improving resource-use efficiency.
In contrast, diurnal species, such as the golden snub-nosed monkey, Temminck’s tragopan, and blood pheasant, were mainly active during daylight hours. Primates generally rely heavily on vision for feeding and social behaviors and therefore typically exhibit diurnal activity patterns [53]. Similarly, most pheasants tend to forage and move during daytime, which may enhance their ability to detect predators [40]. In this study, the activity peaks of Temminck’s tragopan and blood pheasant were concentrated mainly during early morning to late morning hours, possibly reflecting higher foraging efficiency during cooler morning conditions and reduced activity under warmer afternoon temperatures.
In addition, some species exhibited relatively broad temporal niches. Chinese goral, Siberian weasel, and Sichuan takin showed relatively high activity frequencies during both day and night, representing cathemeral activity patterns. Such broad activity schedules may be associated with high foraging demands, extensive movement ranges, and strong adaptability to complex montane environments. Previous studies have suggested that species with broader activity rhythms often exhibit greater ecological flexibility and are able to adjust activity timing according to resource availability and environmental conditions [54]. Moreover, broader temporal niches may reduce direct temporal competition with other species and improve overall resource utilization efficiency.
Notably, some species also exhibited clear seasonal variation in activity rhythms. For example, Temminck’s tragopan showed increased nocturnal activity during winter, while Tibetan macaques displayed seasonal shifts in activity timing. These findings suggest that some animals in the study area can flexibly adjust their activity strategies in response to environmental changes. Seasonal variation in temperature, food resource availability, and human disturbance intensity may all influence animal activity patterns [30,32]. In high-elevation montane forest ecosystems in particular, winter low temperatures and reduced food resources may force some species to expand their activity periods in order to increase foraging opportunities and energy acquisition.
Furthermore, seasonal adjustments in activity rhythms may also be associated with anthropogenic disturbance. Recent studies have shown that wildlife often increases nocturnal activity in response to human disturbance in order to reduce the risk of human encounters [32,55,56]. Although this study did not directly evaluate the effects of human activities, the increased nocturnal activity observed in some species during winter may be related to seasonal tourism activities or variation in human visitation frequency [57]. Future studies incorporating human activity data are therefore needed to further explore these relationships.
Overall, the animal community in the Baishuihe Nature Reserve exhibited pronounced temporal niche partitioning. Different species reduced temporal overlap through diel segregation, expansion of activity periods, and seasonal adjustments in activity rhythms, thereby facilitating more efficient temporal resource allocation. Such temporal niche differentiation likely reduces interspecific competition and potential interference and may represent an important mechanism supporting the long-term coexistence of multiple species within the reserve.
4.4. Study Limitations, Conservation Implications, and Future Perspectives
Although this study analyzed long-term dynamics of mammal and pheasant communities in the Baishuihe Nature Reserve using camera-trap monitoring data, several limitations should be acknowledged. First, this study used the relative abundance index (RAI) as a proxy for relative abundance. Although the RAI has been widely applied in camera-trap studies and can reflect relative activity intensity and detection probability [20,58], it is influenced by species behavior, movement range, detection probability, and camera placement design and therefore cannot directly represent true population density or absolute population size [19]. In particular, highly mobile or wide-ranging species may exhibit inflated RAI values relative to their actual population size, whereas cryptic or infrequently active species may be underestimated.
Second, the spatial representativeness of the present camera-trap dataset should be interpreted with caution. A comprehensive biodiversity survey conducted in 2010 recorded 96 mammal species and 280 bird species in the Baishuihe National Nature Reserve, whereas the present study detected 17 mammal species and 6 ground-dwelling pheasant species. This difference likely reflects differences in survey objectives, taxonomic scope, sampling methods, and spatial coverage. The present camera-trap survey primarily targeted medium- and large-sized mammals and ground-dwelling pheasants, and camera stations were concentrated in part of the reserve rather than covering all habitat types and elevational zones across the entire protected area. In addition, differences in camera numbers, camera placement locations, and effective monitoring duration among years may have influenced comparisons of species richness and detection frequencies across years. Because the monitoring framework during the early stage was not fully standardized, interannual differences in sampling intensity may have caused the observed community changes to reflect both actual ecological variation and sampling effects [59]. Therefore, our results should be interpreted as representing the camera-trap-detectable assemblage within the monitored area, rather than the complete vertebrate diversity of the entire reserve. Future studies should expand camera-trap coverage to additional areas of the reserve, include under-sampled habitat types and elevational zones, and integrate complementary survey methods to improve the representativeness of biodiversity assessments [60].
Third, this study did not include quantitative annual data on anthropogenic or environmental covariates, including visitor numbers, road access, patrol intensity, local human activity, vegetation change, and climatic variation. The Baishuihe area was managed as a protected area throughout the monitoring period, but we were unable to evaluate whether the intensity or spatial distribution of human activities changed during 2011–2020. Therefore, the observed interannual variation in species records and activity patterns should not be attributed to anthropogenic or climatic drivers without further supporting data. Future studies should integrate camera-trap records with standardized information on human disturbance, management activity, habitat change, and climate to better identify the mechanisms underlying temporal changes in wildlife detections and activity rhythms.
Finally, regarding activity rhythm analysis, this study mainly relied on qualitative summaries of detection records across different time periods, and the analyses of activity patterns and temporal niche partitioning remained relatively coarse. Future studies could incorporate kernel density estimation, overlap coefficients, and temporal niche models to quantitatively assess activity curves and temporal overlap among species [29], thereby providing deeper insights into coexistence mechanisms and temporal resource-use strategies.
Despite these limitations, the present study provides useful baseline information on the composition and temporal dynamics of the camera-trap-detectable mammal and ground-dwelling pheasant assemblage within the monitored area [42]. From a conservation management perspective, the results support the continued standardization of camera-trap monitoring in protected areas, including unified camera deployment protocols, optimized monitoring intervals, permanent station identification, and the establishment of long-term monitoring databases, in order to improve comparability among years and regions [61,62]. Future research could also move beyond descriptive analyses of community structure toward investigations of underlying ecological processes and mechanisms. For example, integrating functional traits, trophic relationships, and species interaction networks may improve understanding of the ecological roles of different functional groups. Occupancy models and random encounter models could also be applied to investigate population dynamics and habitat use of key species in greater detail [63].
Overall, this study provides baseline information on the long-term dynamics and temporal organization of camera-trap-detectable mammals and ground-dwelling pheasants in the Baishuihe Nature Reserve. Continued standardized, spatially expanded, and multi-method monitoring will be essential for supporting biodiversity conservation and ecological management within the Giant Panda National Park and the montane regions of southwestern China.
5. Conclusions
This study used a 10-year camera-trap dataset (2011–2020) to investigate the long-term community dynamics and temporal activity patterns of mammals and ground-dwelling pheasants in the Baishuihe National Nature Reserve, a key montane forest ecosystem in southwestern China. A total of 23 species were recorded, including 17 mammal species and 6 pheasant species, representing multiple trophic and functional groups. Several ungulates, pheasants, and mesocarnivores were consistently detected throughout the monitoring period, indicating that the reserve maintains a relatively intact and stable montane vertebrate community with comparatively high ecological integrity. The rate of newly recorded species declined as cumulative sampling increased, illustrating the influence of monitoring effort on the observed species inventory.
The study further revealed pronounced temporal niche differentiation among sympatric species. Diurnal, nocturnal, and cathemeral activity patterns coexisted within the community, while some species also exhibited seasonal shifts in activity rhythms. These patterns suggest that temporal niche partitioning may play an important role in reducing interspecific competition and facilitating long-term species coexistence in montane forest ecosystems. Although some interannual variation in species composition was observed, the persistence of dominant and common species across years indicates relatively high community stability within the reserve. Overall, the study provides baseline information on the composition and temporal organization of the camera-trap-detectable vertebrate assemblage in the Baishuihe National Nature Reserve. These findings can support future standardized monitoring and conservation management within the Giant Panda National Park and the Mountains of Southwest China.
Author Contributions
Conceptualization, Y.Z. and X.C.; methodology, Y.Z. and X.C.; software, Y.Z. and X.C.; formal analysis, Y.Z.; investigation, T.X., H.T., Y.W., H.H. and C.W.; validation, T.X., H.T., Y.W., H.H. and C.W.; data curation, T.X., H.T., Y.W., H.H. and C.W.; writing—original draft preparation, Y.Z.; writing—review and editing, B.Y. and X.C.; visualization, Y.Z. and X.C.; supervision, B.Y. and X.C.; project administration, B.Y. and X.C.; funding acquisition, B.Y. All authors have read and agreed to the published version of the manuscript.
Funding
This work was supported by the National Natural Science Foundation of China (Grant 32470535), the Special Survey on Wild Animals in Chengdu Area of Giant Panda National Park (Grant N5101012025000862), and the Fundamental Research Funds of China West Normal University (Grant 24KE038).
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
The data that support the findings of this study are available from the corresponding author upon reasonable request.
Acknowledgments
We sincerely acknowledge the support from the Chengdu Administration Branch of Giant Panda National Park and the Sichuan Forestry and Grassland Administration.
Conflicts of Interest
The authors declare no conflicts of interest.
References
- Butchart, S.H.M.; Walpole, M.; Collen, B.; van Strien, A.; Scharlemann, J.P.W.; Almond, R.E.A.; Baillie, J.E.M.; Bomhard, B.; Brown, C.; Bruno, J.; et al. Global Biodiversity: Indicators of Recent Declines. Science 2010, 328, 1164–1168. [Google Scholar] [CrossRef] [Scilit]
- Yang, R.; Dong, X.; Xu, S.; Li, X.; Wang, K.; Ye, Y.; Xiao, W. Unveiling Human Impacts on Global Key Biodiversity Areas: Assessing Disturbance and Fragmentation to Inform Conservation Strategies. Geogr. Sustain. 2025, 6, 100259. [Google Scholar] [CrossRef] [Scilit]
- Gray, C.L.; Hill, S.L.L.; Newbold, T.; Hudson, L.N.; Borger, L.; Contu, S.; Hoskins, A.J.; Ferrier, S.; Purvis, A.; Scharlemann, J.P.W. Local Biodiversity Is Higher inside than Outside Terrestrial Protected Areas Worldwide. Nat. Commun. 2016, 7, 12306. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Geldmann, J.; Barnes, M.; Coad, L.; Craigie, I.D.; Hockings, M.; Burgess, N.D. Effectiveness of Terrestrial Protected Areas in Reducing Habitat Loss and Population Declines. Biol. Conserv. 2013, 161, 230–238. [Google Scholar] [CrossRef] [Scilit]
- Plumptre, A.J.; Baisero, D.; Brooks, T.M.; Buchanan, G.; Butchart, S.H.M.; Bowser, A.; Boyd, C.; Carneiro, A.P.B.; Davies, T.; Elliot, W.; et al. Targeting Site Conservation to Increase the Effectiveness of New Global Biodiversity Targets. One Earth 2024, 7, 11–17. [Google Scholar] [CrossRef] [Scilit]
- Cristiano, A.; Pillay, R.; Ramirez-Delgado, J.P.; Watson, J.E.M.; Venter, O.; Pacifici, M. Role of Protected Areas in Mitigating Range Loss and Local Extinctions of Terrestrial Mammals. Conserv. Biol. 2025, 39, e70092. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, C.; Brodie, J.F.; Kays, R.; Davies, T.J.; Liu, R.; Fisher, J.T.; Ahumada, J.; McShea, W.; Sheil, D.; Agwanda, B.; et al. Global Camera Trap Synthesis Highlights the Importance of Protected Areas in Maintaining Mammal Diversity. Conserv. Lett. 2022, 15, e12865. [Google Scholar] [CrossRef] [Scilit]
- Yuan, R.; Zhang, N.; Zhang, Q. The Impact of Habitat Loss and Fragmentation on Biodiversity in Global Protected Areas. Sci. Total Environ. 2024, 931, 173004. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Brum, F.T.; Graham, C.H.; Costa, G.C.; Hedges, S.B.; Penone, C.; Radeloff, V.C.; Rondinini, C.; Loyola, R.; Davidson, A.D. Global Priorities for Conservation across Multiple Dimensions of Mammalian Diversity. Proc. Natl. Acad. Sci. USA 2017, 114, 7641–7646. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Vynne, C.; Gosling, J.; Maney, C.; Dinerstein, E.; Lee, A.T.L.; Burgess, N.D.; Fernandez, N.; Fernando, S.; Jhala, H.; Jhala, Y.; et al. An Ecoregion-Based Approach to Restoring the World’s Intact Large Mammal Assemblages. Ecography 2022, 2022, 1–12. [Google Scholar] [CrossRef] [Scilit]
- Pacifici, M.; Di Marco, M.; Watson, J.E.M. Protected Areas Are Now the Last Strongholds for Many Imperiled Mammal Species. Conserv. Lett. 2020, 13, e12748. [Google Scholar] [CrossRef] [Scilit]
- Feng, Y.; Cao, Y.; Chan, M.Y.; Ye, Z.; Zhao, Z.; Yu, L.; Liang, Y.; Carver, S.; Yang, R. Assessing Ecosystem Integrity in Protected Areas: A Systematic Review of Methods and Applications. Biol. Conserv. 2025, 305, 111057. [Google Scholar] [CrossRef] [Scilit]
- Torretta, E.; Serafini, M.; Puopolo, F.; Schenone, L. Spatial and Temporal Adjustments Allowing the Coexistence among Carnivores in Liguria (N-W Italy). Acta Ethologica 2016, 19, 123–132. [Google Scholar] [CrossRef] [Scilit]
- Nagy-Reis, M.B.; Iwakami, V.H.S.; Estevo, C.A.; Setz, E.Z.F. Temporal and Dietary Segregation in a Neotropical Small-Felid Assemblage and Its Relation to Prey Activity. Mamm. Biol. 2019, 95, 1–8. [Google Scholar] [CrossRef] [Scilit]
- Mori, E.; Bagnato, S.; Serroni, P.; Sangiuliano, A.; Rotondaro, F.; Marchiano, V.; Cascini, V.; Poerio, L.; Ferretti, F. Spatiotemporal Mechanisms of Coexistence in an European Mammal Community in a Protected Area of Southern Italy. J. Zool. 2020, 310, 232–245. [Google Scholar] [CrossRef] [Scilit]
- Karanth, K.U.; Srivathsa, A.; Vasudev, D.; Puri, M.; Parameshwaran, R.; Kumar, N.S. Spatio-Temporal Interactions Facilitate Large Carnivore Sympatry across a Resource Gradient. Proc. R. Soc. B Biol. Sci. 2017, 284, 20161860. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Smith, J.A.; Thomas, A.C.; Levi, T.; Wang, Y.; Wilmers, C.C. Human Activity Reduces Niche Partitioning among Three Widespread Mesocarnivores. Oikos 2018, 127, 890–901. [Google Scholar] [CrossRef] [Scilit]
- Diao, Y.; Zhao, Q.; Weng, Y.; Gu, B.; Wang, F. Temporal Shifts as Elusive Responses to Anthropogenic Stressors in a Mammal Community. Biodivers. Conserv. 2021, 30, 2529–2544. [Google Scholar] [CrossRef] [Scilit]
- Gilbert, N.A.; Clare, J.D.J.; Stenglein, J.L.; Zuckerberg, B. Abundance Estimation of Unmarked Animals Based on Camera-Trap Data. Conserv. Biol. 2021, 35, 88–100. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Burton, A.C.; Neilson, E.; Moreira, D.; Ladle, A.; Steenweg, R.; Fisher, J.T.; Bayne, E.; Boutin, S. Wildlife Camera Trapping: A Review and Recommendations for Linking Surveys to Ecological Processes. J. Appl. Ecol. 2015, 52, 675–685. [Google Scholar] [CrossRef] [Scilit]
- Hoffman, M.; Koenig, K.; Bunting, G.; Costanza, J.; Williams, K.J. Biodiversity Hotspots (Version 2016.1) 2016. Available online: https://cir.nii.ac.jp/crid/1881428067530588032 (accessed on 20 July 2026).
- Oliver, R.Y.; Iannarilli, F.; Ahumada, J.; Fegraus, E.; Flores, N.; Kays, R.; Birch, T.; Ranipeta, A.; Rogan, M.S.; Sica, Y.V.; et al. Camera Trapping Expands the View into Global Biodiversity and Its Change. Philos. Trans. R. Soc. B-Biol. Sci. 2023, 378, 20220232. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, X.; Tian, T.; Pan, H.; Jin, Y.; Zhang, X.; Xiang, Y.; Yang, B.; Zhang, L. Coexistence Mechanisms of Small Carnivores in a Near-Pristine Area within the Mountains of Southwest China. Glob. Ecol. Conserv. 2024, 49, e02777. [Google Scholar] [CrossRef] [Scilit]
- Palencia, P.; Vicente, J.; Soriguer, R.C.; Acevedo, P. Towards a Best-Practices Guide for Camera Trapping: Assessing Differences among Camera Trap Models and Settings under Field Conditions. J. Zool. 2022, 316, 197–208. [Google Scholar] [CrossRef] [Scilit]
- Colyn, R.B.; Radloff, F.G.T.; O’Riain, M.J. Camera Trapping Mammals in the Scrubland’s of the Cape Floristic Kingdom-the Importance of Effort, Spacing and Trap Placement. Biodivers. Conserv. 2018, 27, 503–520. [Google Scholar] [CrossRef] [Scilit]
- O’Brien, T.G.; Kinnaird, M.F.; Wibisono, H.T. Crouching Tigers, Hidden Prey: Sumatran Tiger and Prey Populations in a Tropical Forest Landscape. Anim. Conserv. 2003, 6, 131–139. [Google Scholar] [CrossRef] [Scilit]
- Baselga, A. Partitioning the Turnover and Nestedness Components of Beta Diversity. Glob. Ecol. Biogeogr. 2010, 19, 134–143. [Google Scholar] [CrossRef] [Scilit]
- Colwell, R.K.; Coddington, J.A. Estimating Terrestrial Biodiversity Through Extrapolation. Philos. Trans. R. Soc. B-Biol. Sci. 1994, 345, 101–118. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ridout, M.S.; Linkie, M. Estimating Overlap of Daily Activity Patterns From Camera Trap Data. J. Agric. Biol. Environ. Stat. 2009, 14, 322–337. [Google Scholar] [CrossRef] [Scilit]
- Frey, S.; Fisher, J.T.; Burton, A.C.; Volpe, J.P. Investigating Animal Activity Patterns and Temporal Niche Partitioning Using Camera-Trap Data: Challenges and Opportunities. Remote Sens. Ecol. Conserv. 2017, 3, 123–132. [Google Scholar] [CrossRef] [Scilit]
- Kronfeld-Schor, N.; Dayan, T. Partitioning of Time as an Ecological Resource. Annu. Rev. Ecol. Evol. Syst. 2003, 34, 153–181. [Google Scholar] [CrossRef] [Scilit]
- Gaynor, K.M.; Hojnowski, C.E.; Carter, N.H.; Brashares, J.S. The Influence of Human Disturbance on Wildlife Nocturnality. Science 2018, 360, 1232–1235. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Schoener, T.W. Resource Partitioning in Ecological Communities. Science 1974, 185, 27–39. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hoeks, S.; Huijbregts, M.A.J.; Busana, M.; Harfoot, M.B.J.; Svenning, J.-C.; Santini, L. Mechanistic Insights into the Role of Large Carnivores for Ecosystem Structure and Functioning. Ecography 2020, 43, 1752–1763. [Google Scholar] [CrossRef] [Scilit]
- Refinetti, R. The Diversity of Temporal Niches in Mammals. Biol. Rhythm Res. 2008, 39, 173–192. [Google Scholar] [CrossRef] [Scilit]
- Ripple, W.J.; Estes, J.A.; Beschta, R.L.; Wilmers, C.C.; Ritchie, E.G.; Hebblewhite, M.; Berger, J.; Elmhagen, B.; Letnic, M.; Nelson, M.P.; et al. Status and Ecological Effects of the World’s Largest Carnivores. Science 2014, 343, 1241484. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tobler, M.W.; Carrillo-Percastegui, S.E.; Pitman, R.L.; Mares, R.; Powell, G. An Evaluation of Camera Traps for Inventorying Large- and Medium-Sized Terrestrial Rainforest Mammals. Anim. Conserv. 2008, 11, 169–178. [Google Scholar] [CrossRef] [Scilit]
- Marneweck, C.; Butler, A.R.; Gigliotti, L.C.; Harris, S.N.; Jensen, A.J.; Muthersbaugh, M.; Newman, B.A.; Saldo, E.A.; Shute, K.; Titus, K.L.; et al. Shining the Spotlight on Small Mammalian Carnivores: Global Status and Threats. Biol. Conserv. 2021, 255, 109005. [Google Scholar] [CrossRef] [Scilit]
- Wehr, N.H.; Boone, H.M.; van den Bosch, M.; Zubiria Perez, A.; Wehr, K.L.; Wehr, S.R.; Belant, J.L. Interspecific Carnivore Competition and Ungulate Predation Correlate with Predator Species Richness. Ecology 2025, 106, e70136. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pheasants in China. Available online: https://www.nhbs.com/pheasants-in-china-chinese-book (accessed on 27 May 2026). (In Chinese)
- Lindenmayer, D.B.; Gibbons, P.; Bourke, M.; Burgman, M.; Dickman, C.R.; Ferrier, S.; Fitzsimons, J.; Freudenberger, D.; Garnett, S.T.; Groves, C.; et al. Improving Biodiversity Monitoring. Austral Ecol. 2012, 37, 285–294. [Google Scholar] [CrossRef] [Scilit]
- White, E.R. Minimum Time Required to Detect Population Trends: The Need for Long-Term Monitoring Programs. Bioscience 2019, 69, 40–46. [Google Scholar] [CrossRef] [Scilit]
- Harmsen, B.J.; Saville, N.; Foster, R.J. Long-Term Monitoring of Margays (Leopardus Wiedii): Implications for Understanding Low Detection Rates. PLoS ONE 2021, 16, e0247536. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Blondel, J. Guilds or Functional Groups: Does It Matter? Oikos 2003, 100, 223–231. [Google Scholar] [CrossRef] [Scilit]
- Olesen, J.M.; Stefanescu, C.; Traveset, A. Strong, Long-Term Temporal Dynamics of an Ecological Network. PLoS ONE 2011, 6, e26455. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Magurran, A.E.; Henderson, P.A. Explaining the Excess of Rare Species in Natural Species Abundance Distributions. Nature 2003, 422, 714–716. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jain, M.; Flynn, D.F.B.; Prager, C.M.; Hart, G.M.; DeVan, C.M.; Ahrestani, F.S.; Palmer, M.I.; Bunker, D.E.; Knops, J.M.H.; Jouseau, C.F.; et al. The Importance of Rare Species: A Trait-Based Assessment of Rare Species Contributions to Functional Diversity and Possible Ecosystem Function in Tall-Grass Prairies. Ecol. Evol. 2014, 4, 104–112. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Saterberg, T.; Jonsson, T.; Yearsley, J.; Berg, S.; Ebenman, B. A Potential Role for Rare Species in Ecosystem Dynamics. Sci. Rep. 2019, 9, 11107. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dornelas, M.; Gotelli, N.J.; McGill, B.; Shimadzu, H.; Moyes, F.; Sievers, C.; Magurran, A.E. Assemblage Time Series Reveal Biodiversity Change but Not Systematic Loss. Science 2014, 344, 296–299. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jenks, K.E.; Chanteap, P.; Damrongchainarong, K.; Cutter, P.; Cutter, P.; Redford, T.; Lynam, A.J.; Howard, J.; Leimgruber, P. Using Relative Abundance Indices from Camera-Trapping to Test Wildlife Conservation Hypotheses—An Example from Khao Yai National Park, Thailand. Trop. Conserv. Sci. 2011, 4, 113–131. [Google Scholar] [CrossRef] [Scilit]
- Moore, J.F.; Pine, W.E.; Mulindahabi, F.; Niyigaba, P.; Gatorano, G.; Masozera, M.K.; Beaudrot, L. Comparison of Species Richness and Detection between Line Transects, Ground Camera Traps, and Arboreal Camera Traps. Anim. Conserv. 2020, 23, 561–572. [Google Scholar] [CrossRef] [Scilit]
- Noor, A.; Mir, Z.R.; Veeraswami, G.G.; Habib, B. Activity Patterns and Spatial Co-Occurrence of Sympatric Mammals in the Moist Temperate Forest of the Kashmir Himalaya, India. Folia Zool. 2017, 66, 231–241. [Google Scholar] [CrossRef] [Scilit]
- Guo, S.; Li, B.; Watanabe, K. Diet and Activity Budget of Rhinopithecus Roxellana in the Qinling Mountains, China. Primates 2007, 48, 268–276. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Monterroso, P.; Alves, P.C.; Ferreras, P. Plasticity in Circadian Activity Patterns of Mesocarnivores in Southwestern Europe: Implications for Species Coexistence. Behav. Ecol. Sociobiol. 2014, 68, 1403–1417. [Google Scholar] [CrossRef] [Scilit]
- Frey, S.; Volpe, J.P.; Heim, N.A.; Paczkowski, J.; Fisher, J.T. Move to Nocturnality Not a Universal Trend in Carnivore Species on Disturbed Landscapes. Oikos 2020, 129, 1128–1140. [Google Scholar] [CrossRef] [Scilit]
- Liu, M.; McShea, W.J.; Hua, F.; Guan, T.; Wang, D.; Shen, X.; Li, S. Effects of Protected Areas on Human-Induced Shifts in Nocturnal Activity in Mammal Communities in Southwestern China. Conserv. Biol. 2026, 40, e70188. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Seveque, A.; Gentle, L.K.; Lopez-Bao, J.V.; Yarnell, R.W.; Uzal, A. Human Disturbance Has Contrasting Effects on Niche Partitioning within Carnivore Communities. Biol. Rev. 2020, 95, 1689–1705. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- O’Brien, T.G.; Baillie, J.E.M.; Krueger, L.; Cuke, M. The Wildlife Picture Index: Monitoring Top Trophic Levels. Anim. Conserv. 2010, 13, 335–343. [Google Scholar] [CrossRef] [Scilit]
- Heiniger, J.; Gillespie, G. High Variation in Camera Trap-Model Sensitivity for Surveying Mammal Species in Northern Australia. Wildl. Res. 2018, 45, 578–585. [Google Scholar] [CrossRef] [Scilit]
- McIntyre, T.; Majelantle, T.L.; Slip, D.J.; Harcourt, R.G. Quantifying Imperfect Camera-Trap Detection Probabilities: Implications for Density Modelling. Wildl. Res. 2020, 47, 177–185. [Google Scholar] [CrossRef] [Scilit]
- Ferreras, P.; Diaz-Ruiz, F.; Alves, P.C.; Monterroso, P. Optimizing Camera-Trapping Protocols for Characterizing Mesocarnivore Communities in South-Western Europe. J. Zool. 2017, 301, 23–31. [Google Scholar] [CrossRef] [Scilit]
- Bruce, T.; Amir, Z.; Allen, B.L.; Alting, B.F.; Amos, M.; Augusteyn, J.; Ballard, G.-A.; Behrendorff, L.M.; Bell, K.; Bengsen, A.J.; et al. Large-Scale and Long-Term Wildlife Research and Monitoring Using Camera Traps: A Continental Synthesis. Biol. Rev. 2025, 100, 530–555. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Royle, J.A.; Chandler, R.B.; Sollmann, R.; Gardner, B. Spatial Capture-Recapture; Academic Press: Waltham, MA, USA, 2013; ISBN 978-0-12-405939-9. [Google Scholar]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.