


Abstract
(1) The prevalence of depression is two times higher in women than men. Black women have an increased risk of depression due to stressors such as low socioeconomic status and perceived discrimination. Depression is likely influenced by both genetic and environmental factors. Psychosocial stressors can influence DNA methylation (DNAm), leading to changes in gene expression and ultimately, depression. The objective of this study was to examine associations between DNAm and depressive symptoms in Black women. (2) This study was a secondary analysis of data from the Intergenerational Impact of Genetic and Psychological Factors on Blood Pressure (InterGEN) Study. Perceived discrimination was assessed using Krieger’s Experiences of Discrimination and Waelde’s Race-Related Events Scale, and participants were screened for depressive symptoms with the Beck Depression Inventory. Raw data from saliva samples were analyzed using the Illumina Infinium Epic (850 K) BeadChip and then preprocessed in RStudio. (3) Differential methylation analysis identified DNAm sites and regions associated with depressive symptoms. Six DNAm sites had a q-value less than 0.05. Additionally, of the 25 regions identified, 12 were associated with neurological diseases or disorders. (4) These findings suggest that there is a neurological component to depression, which should be considered during treatment.
1. Introduction
Depression affects over 350 million people globally and is ranked second in worldwide disease burden; it is expected to rank first by 2030 [1,2]. The prevalence of depression peaks in the second and third decades of life and is roughly two times higher in women (24.0%) compared to men (13.3%) in the United States (US), which may be partly due to the willingness of women to report symptoms [1,3,4]. Depression is driven by both social and biological factors, many of which have been poorly elucidated, and largely attributed to differences in reporting bias between sexes [3].
Black women are a group that is at a very high risk of developing depression because they are more likely to be the single head of the household; living in a poorer, higher crime neighborhood; bearing the burden of caring for family members; and dealing with discrimination [5]. Black women are also more likely to be of a lower socioeconomic status [6]. In the US National Survey of American Life, 21.3% of Black women reported depression compared to 10.1% of White women [7]. In addition, the Study of Environment, Lifestyle, and Fibroids (SELF), which focuses on Black women, reported symptoms of depression in 43% of participants [8]. Black women are sometimes unaware of their symptoms of depression due to cultural coping [5]. There is also a stigma related to depression in the Black community, and depression can be seen as a sign of weakness, leading to the reluctance of Black women to report symptoms [5]. Even when diagnosed with depression, Black women have more severe and chronic disease [9].
Depression is characterized by symptoms such as low mood, feelings of worthlessness or hopelessness, anhedonia, appetite changes, sleep disturbances, and suicidal ideation [10]. Women are more likely to report symptoms like weight gain, increase in appetite, and somatic symptoms [3]. Women are also more likely to experience social disadvantages than men [3]. Many hormones impact the risk of depression, including testosterone, estrogen, serotonin, and cortisol [11]. These hormones vary throughout the lifespan and interact with social factors, putting some groups at higher risk than others of developing depression [12]. In addition, the production of these hormones can change in response to stress and affect cognitive and emotional function [11].
Diagnosing depression can be difficult due to the varied symptom presentations and complicated etiology [13]. A formal diagnosis of depression is generally made by a trained mental health professional who identifies symptoms based on the Diagnostic and Statistical Manual of Mental Disorders or the International Classification of Diseases [1]. Individuals may also be screened for depressive symptoms using measurement instruments designed for this purpose, which can be self-administered [1]. However, some people may not have access to a trained professional, or stigma may prevent them from seeking care [14]. Patients may also be reluctant to divulge sensitive information to providers [15]. For these reasons, screening and diagnosis are difficult, and many people remain undiagnosed and untreated [5].
The utilization of genetic data is being explored as a more objective method for diagnosis. Depression has an estimated heritability of approximately 40%, and both genetic and environmental factors likely contribute to depression [2,16]. The complex interplay between societal factors that are known to impact depression—systemic racism, discrimination, and socioeconomic deprivation—interacts with underlying biological factors (e.g., genes) to increase stress, leading to epigenetic changes and ultimately depression [17,18]. DNA methylation is an epigenetic modification that can affect gene expression without altering DNA sequences [19]. These modifications are responsive to environmental stimuli and may be reversible [19]. Psychosocial stressors, such as experiences with discrimination, have been shown to influence DNA methylation, leading to changes in gene expression [13].
Other studies have investigated the association between DNA methylation and depression [19,20]. Differential methylation related to depression has been observed in several genes, including BDNF, NTRK2, SLC6A4, NR3C1, PRIMA1, and OXTR, but results across studies are inconsistent [19,21]. However, no studies have investigated the relationship between DNA methylation and depression in Black women. Therefore, the objective of this study is to examine associations between DNA methylation and depressive symptoms in Black women.
2. Results
Individual characteristics are summarized in Table 1. A total of 235 women had usable DNA methylation data and complete responses on the BDI. The average age was 31, and 8% were Hispanic or Latino. Approximately 5% had some high school education, and 36% had a high school diploma or general educational diploma (GED). Over half of the participants (65%) were single. Nearly half (45%) reported an annual household income of less than USD 15,000. Unemployment benefits were received by 23%, 3% received Temporary Assistance for Needy Families (TANF) or Family Investment Program (FIP), and 3% reported no cash income. Over a quarter of participants (28%) reported receiving food stamps, 23% received a housing subsidy, 17% received heating assistance, and 17% received Women, Infants, and Children (WIC) benefits. Only 18% reported always having money for basic things, and 40% responded with “most of the time”. When asked how often they have money for special things, 13% of participants responded with “never”, and 44% responded with “sometimes”. Over half (61%) of participants had Medicaid insurance, and 5% had no insurance. Approximately one-fifth (21%) were not living in permanent housing at the time of the interview. Depressive symptoms were categorized into four levels: normal (n = 159), mild to moderate (n = 45), moderate to severe (n = 18), and severe (n = 13). Nearly a third (32%) of participants reported experiencing depressive symptoms at a level higher than normal.
Table 1.
Participant Characteristics.
Bivariate associations were examined between participant characteristics and depression symptoms (Table 1). Depressive symptoms were significantly associated with household income, type of cash income, type of non-cash income, whether participants had money for basic things or special things, EOD scores, and RRES scores.
When participants were stratified by severity of depressive symptoms, there was a significant difference in marital status between groups (p = 0.003) with a higher percentage of the moderate-to-severe and severe groups reporting single marital status (Table S1). A larger proportion of the severe group reported no cash income and a smaller proportion of this group indicated receiving employment income. Unemployment benefits were received by a larger proportion of the mild-to-moderate, moderate-to-severe, and severe groups. More of the mild-to-moderate group received food stamps. A larger portion of the groups reporting depressive symptoms indicated having money for basic things only sometimes or about half the time; a larger portion of these groups also reported never having money for special things. More of the mild-to-moderate and moderate-to-severe participants reported not living in permanent housing at the time of the interview. The group reporting a severe level of depressive symptoms had significantly higher scores on the EOD and RRES than the normal group.
Differentially methylated CpG sites associated with depressive symptoms were identified using dmpFinder. A total of six CpG sites were identified with a q-value less than 0.05 (Table 2). However, none of these sites were annotated to a gene; all were located in noncoding regions.
Table 2.
Significant CpG Sites Associated with Level of Depressive Symptoms.
Bumphunter identified 25 differentially methylated regions associated with depressive symptoms (Table 3). These regions were annotated to nearby genes and were located inside introns (n = 16), inside exons (n = 3), downstream (n = 1), or upstream from the gene (n = 4), or in the promoter region (n = 1). The regions inside introns, like the significant CpGs in Table 2, were noncoding. Twelve of the nearby genes were associated with neurological diseases or disorders, including spasticity, neuroblastoma, and neuropathy [22]. Five of the genes were involved in neurological pathways, and two genes had a neurologically related function [22].
Table 3.
Annotation of Differentially Methylated Regions Associated with Level of Depressive Symptoms.
3. Discussion
In this secondary analysis of data from the InterGEN study, we identified relationships between depressive symptoms and six differentially methylated positions, and twenty-five differentially methylated regions associated with depressive symptoms. In this study, a total of 12 annotated genes were associated with neurological diseases: GLRX5, CLEC1B, NBPF8, NDUFA10, PLEKHM3, L3MBTL4, ADCY8, ARHGEF10, TAFA5, OTOF, TANGO2, and LINC02915. Two of the annotated genes have a direct neurological impact: CLEC1B is involved in the process of cognition, and PKD1L3 functions in the reception of the sense of taste [22].
Glutaredoxin 5 (GLRX5) has been associated with neuromuscular spasticity and neuroimaging abnormalities [23]. The CLEC1B gene was found to be correlated with cognitive function [24] and bipolar disorder in humans [25]. It has also been associated with bipolar disorder in an analysis of cerebrospinal fluid [25]. Neuroblastoma Breakpoint Family genes, such as NBPF8, are associated with neuroblastoma, a cancer that arises from nerve cells, often in the sympathetic nervous system [26].
The NDUFA10 gene has been linked to Leigh syndrome, a neurogenerative disease characterized by lesions in the basal ganglia and/or brainstem and deficits in motor function [27]. This gene also functions in the biogenesis of mitochondrial complex I; dysfunction in the mitochondria can lead to neurological disorders such as seizures, dystonia, ataxia, optic atrophy, and sensorineural hearing loss [28]. The PLEKHM3 gene has been associated with neuropathy and chordoma [22].
The L3MBTL4 gene has been linked to N Syndrome, which can cause seizures, nystagmus, spasticity, and severe intellectual impairment, and Bardet–Biedl Syndrome, which often presents with visual and intellectual impairments [29,30]. Adenylate cyclase 8 (ADCY8) functions in the regulation of synapse activity and has been associated with dissociative amnesia [22,31]. Rho Guanine Nucleotide Exchange Factor 10 (ARHGEF10) has previously been linked to nerve conduction velocity, neuropathy, and elevated risk of ischemic stroke [22,32]. In mice, the TAFA5 gene was associated with depression and was expressed in brain tissue [33].
The otoferlin gene (OTOF) functions in the sensory processing of sound and smell [22]. It has been associated with autosomal recessive deafness and auditory neuropathy [22,34]. TANGO2 has been linked to neurodegeneration and encephalopathy [18]. Deficiencies in this gene can lead to developmental delays, intellectual disability, spasticity, gait abnormality, speech impairment, and seizures [35]. LINC02915 is noncoding and located in an intron, but it has been associated with spastic paraplegia [22].
With the exception of TAFA5, none of these genes have previously been associated with depression. However, their association with depressive symptoms in this study and the related neurological functions suggest possible links between depression and the neurological system. Depression has previously been classified as both a mental illness and a neurological or neuropsychiatric disorder and is often treated by influencing the levels of neurotransmitters in the brain, such as serotonin, norepinephrine, and dopamine [36,37]. However, as many individuals fail to respond to traditional pharmacological therapies, treatments directly targeting the brain are being implemented, such as transcranial magnetic stimulation, electroconvulsive therapy, and vagus nerve stimulation [37]. In addition, depressive episodes have been induced during high-frequency stimulation of the substantia nigra in patients with no prior psychiatric history, and positron emission tomography performed during a depressive episode showed dysfunctional circuitry between cortical and subcortical regions of the brain [38]. Low self-esteem, one of the common symptoms of depression, has been associated with decreased neural activity in the amygdala in functional magnetic resonance imaging studies [39].
This disorder has also been associated with increased levels of inflammatory cytokines, which can negatively affect pathways associated with mood, emotion, and cognition, such as neurotransmission, activation of microglia, dysregulation of the hypothalamic–pituitary–adrenal axis, and brain plasticity [40]. In a transcriptomic study of depression using RNA-Seq analysis of samples of microglia from the prefrontal cortex, there were significant differences between samples from depressed individuals and healthy controls [41]. In addition, this study found significant changes in signaling pathways related to cell communication, cell adhesion, cell growth, and differentiation [41]. Continued emphasis on the neurological aspects of depression could lead to novel discoveries in the pathology of this disorder, improvements in drug development and repurposing, and advances in precision medicine for individuals with depression.
Limitations
There were a few limitations to this study. The participants were all healthy with some reporting depressive symptoms during screening. Analyzing the DNAm of a sample of depressed participants could identify additional differential methylation. Depressive symptoms were assessed in the current study using the BDI. Ideally, as many depressive symptom scales exist, multiple scales should be used to screen participants, and their associated genes can be compared for consistency [42].
In addition, sequencing was performed using saliva samples. Prior research has suggested that epigenetic changes associated with depression are more enriched in neuronal cells [19]. The genes associated with depression in previous studies may not have been replicated in this study because previous studies of epigenetics and depression were not conducted on a sample of Black women. A systematic review of 67 DNAm studies focusing on depression included studies performed in the US, Australia, Asia, and Europe, but did not include any studies performed in Africa [20]. In addition, some studies only focused on one or a few candidate genes while the current study used an epigenome-wide approach [19,20]. Many of the included studies reported no associations at all with depression [20].
The different studies did not all recruit study participants with the same depression phenotype; different phenotypes included major depressive disorder, postpartum depression, “depression in general”, and depressive symptoms [20]. Sample types were also inconsistent and included whole blood, buccal cells, leukocytes, brain tissue, saliva and peripheral blood mononuclear cells [20]. These varied results and methods indicate that associations are difficult to replicate across studies. Future research should focus on more diverse populations and include more depressed individuals to compare with healthy controls. It would also be helpful for researchers to establish a gold-standard sample type because different cell types can yield different results [19]. While prior research has suggested that neuronal cells are ideal for showing DNAm changes, this sample type is more difficult to obtain from live participants than from blood or saliva [19]. Future research could also include brain imaging of study participants to pinpoint differences between individuals with depression and healthy controls or to identify depression subtypes [39].
4. Materials and Methods
4.1. Theoretical Framework
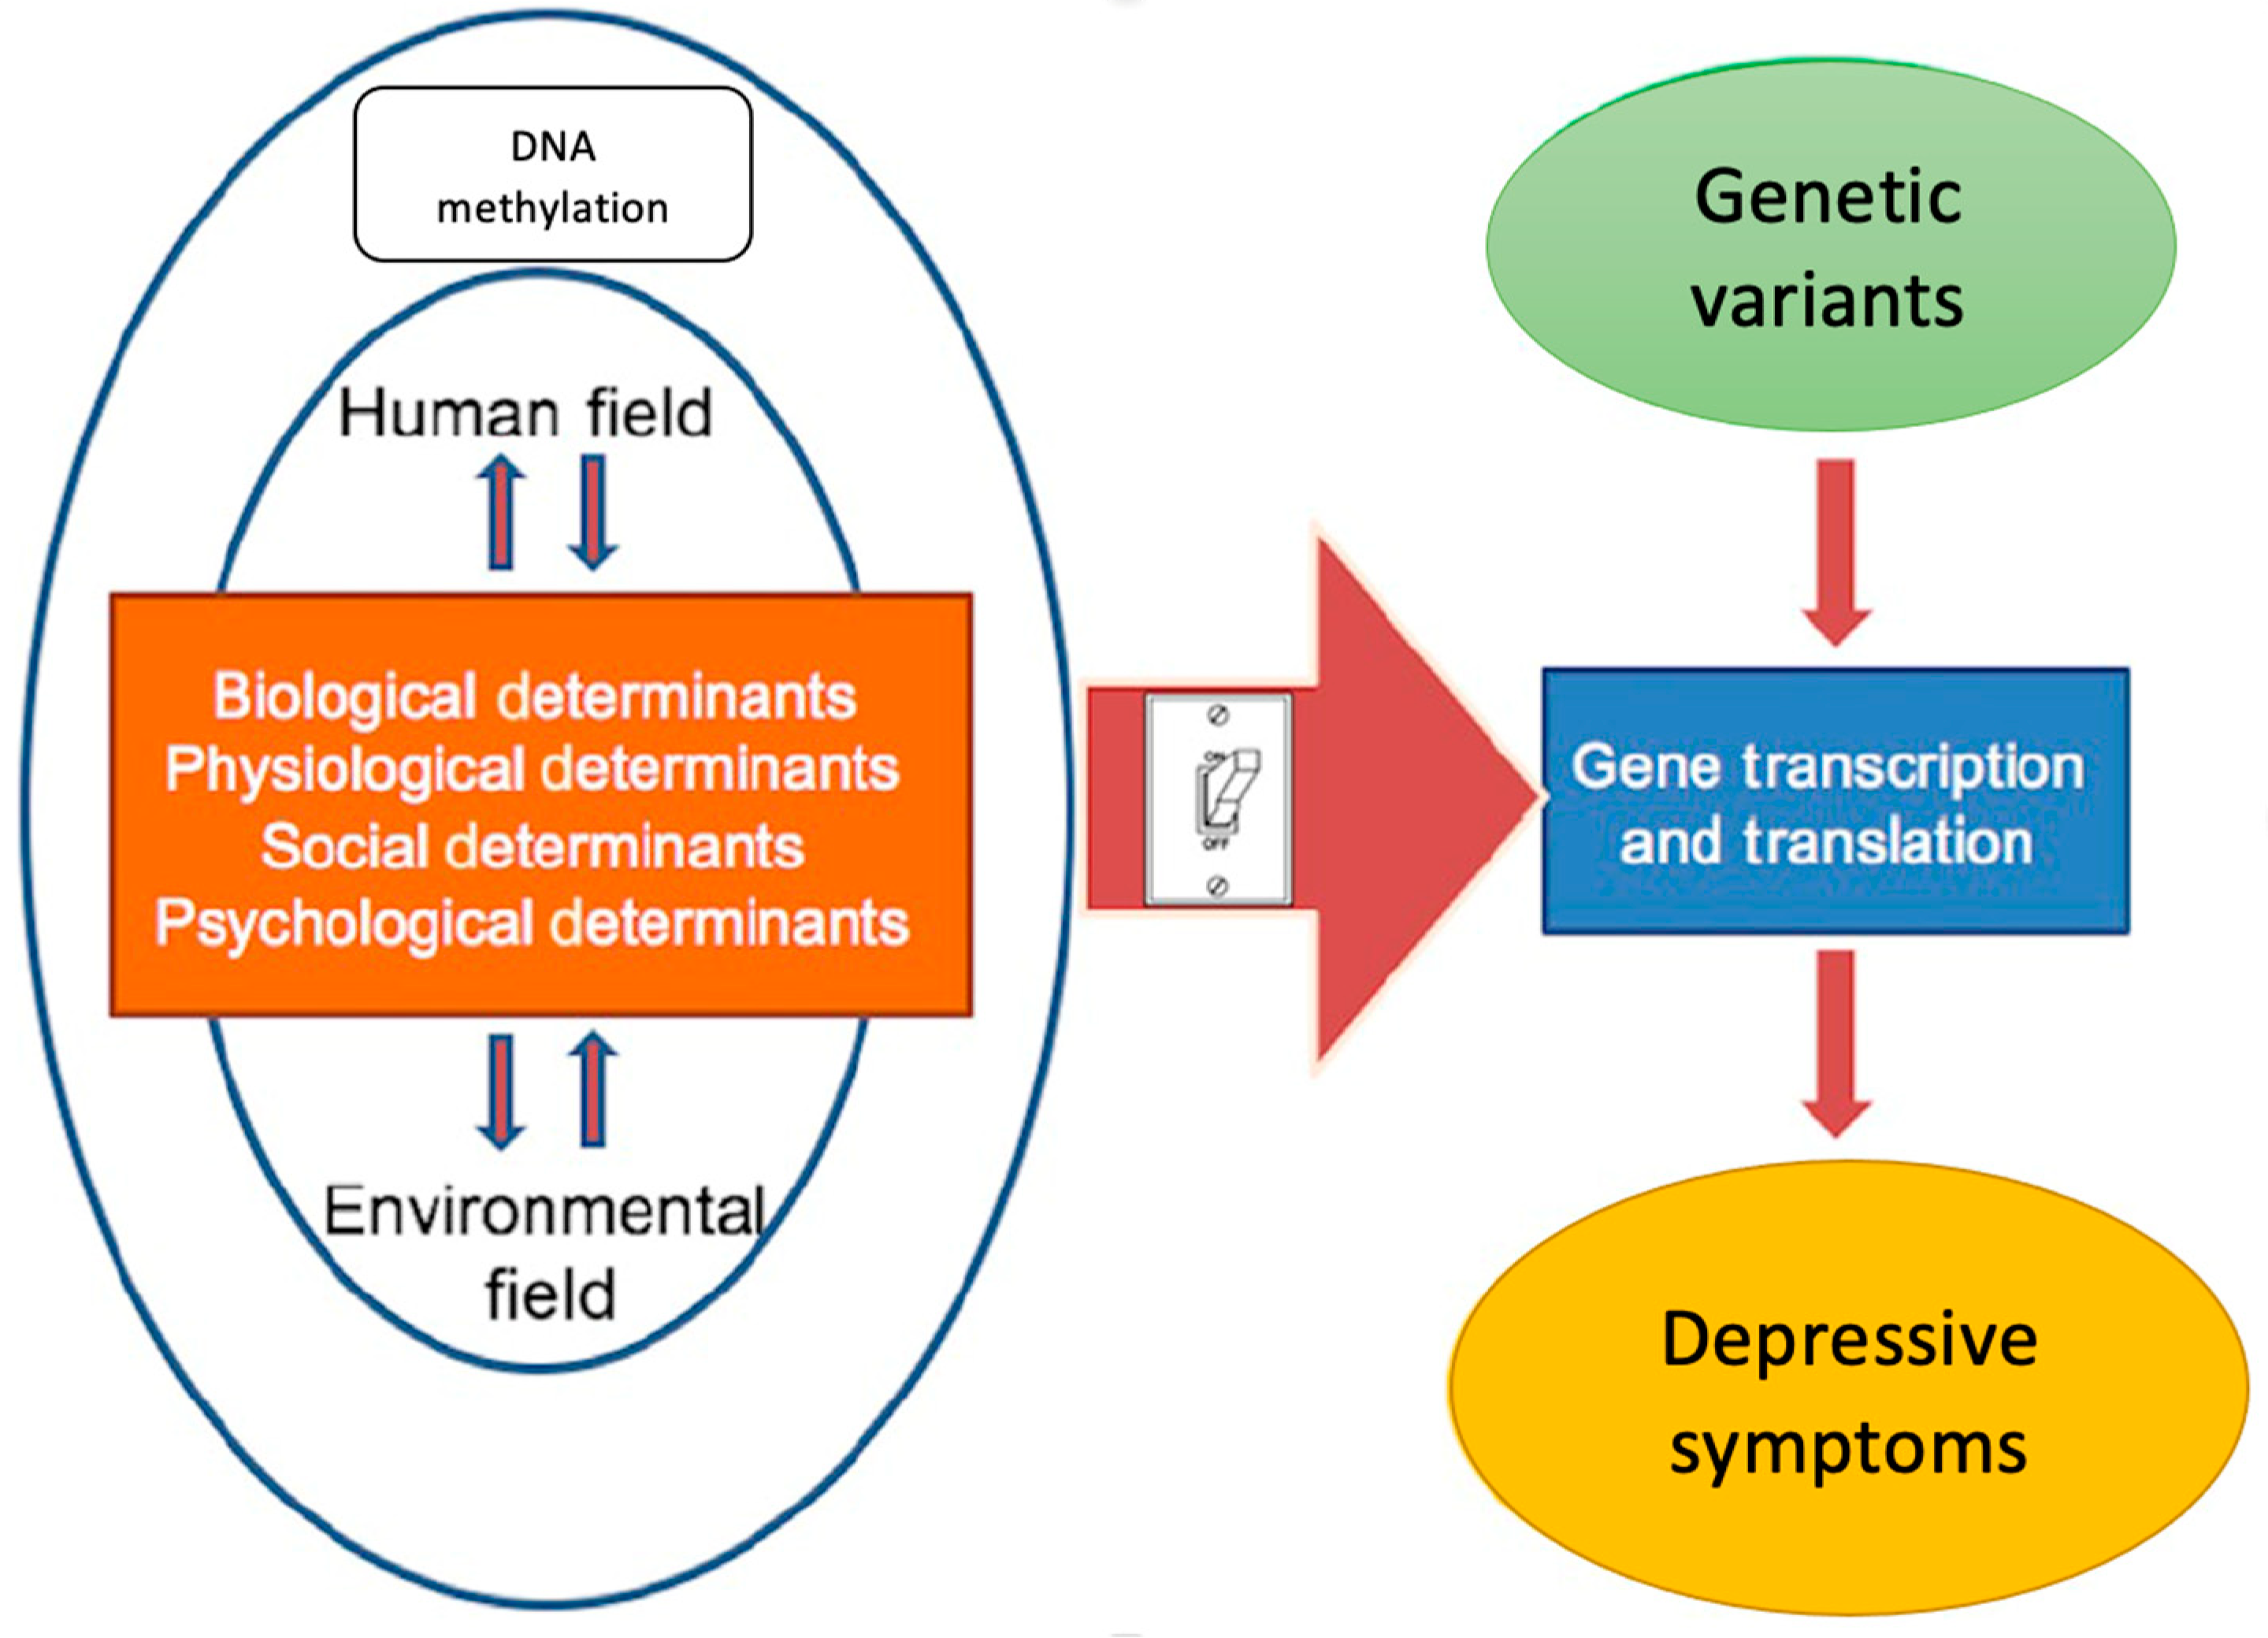
This study was guided by the University of Illinois at Chicago (UIC) Model for Genetic and Epigenetic Research (Figure 1), which asserts that genetic and environmental influences interact and lead to a phenotype [43].
Figure 1.
Adapted UIC Model for Genetic and Epigenetic Research.
Humans constantly interact with their environment, and these interactions can affect health status [43]. Biological, physiological, social, and psychological factors can influence DNA methylation and gene expression, leading to depressive symptoms.
4.2. Study Design and Sample
We conducted a secondary analysis of data from the Intergenerational Impact of Genetic and Psychological Factors on Blood Pressure (InterGEN) study. This study was a longitudinal study of Black mothers and their children aged 3–5 [44]. The aim was to examine the effects of gene-environment interaction on blood pressure in Black women and their children [44]. Participants were recruited from early childhood education centers and community events in Southwest and Central Connecticut from 2014 to 2019 [44]. Inclusion criteria are women aged 21 or older with a biological child aged 3 to 5 years, who identify as Black or African American, are fluent in English, and have not been diagnosed with a psychiatric or cognitive disorder that could affect the reporting of data [44].
Interviews were conducted at four time points, and information on demographics and social determinants of health and measurements of physical health were collected at each interview [44]. Demographics and information on social determinants of health were obtained in face-to-face interviews using Audio Computer-Assisted Self-Interviewing [44]. In this interviewing method, questions and responses are displayed on the computer screen, and participants can hear the question via audio [44].
4.3. Instruments and Measures
4.3.1. Sociodemographic Variables
Sociodemographic variables included age, ethnicity, marital status, income, education, insurance status, and housing. All participants were female and self-identified their race as Black or African American. The categories for marital status were married, single, divorced, separated, or living with but not married to a significant other. Education levels were less than high school, high school diploma or GED, some college, associate’s degree, bachelor’s degree, master’s degree, or doctorate. Health insurance response options were insured or uninsured, and housing options were permanent or nonpermanent housing.
4.3.2. Depressive Symptoms
Symptoms of depression were assessed at each interview using the Beck Depression Inventory (BDI) [45]. This scale contains 21 items, each of which describes a specific symptom of depression: mood, pessimism, feelings of failure, lack of satisfaction, feelings of guilt, sense of punishment, self-hate, self-accusations, self-punitive wishes, crying spells, irritability, social withdrawal, body image issues, work inhibition, sleep disturbances, fatigue, appetite changes, weight changes, somatic preoccupation, and loss of libido [46]. Each item contains four to six ordinal statements meant to reflect the severity of the symptom from neutral to maximum severity [45]. The statements are assigned numerical values from 0 to 3, and the scores for each statement are summed into a total score [45]. The severity of depressive symptoms is classified as follows: <10 is none or minimal; 10–18 is mild to moderate; 19–29 is moderate to severe; and 30–63 is severe [46].
4.3.3. Perceived Discrimination
Two instruments were used to assess perceived discrimination: the Experiences of Discrimination (EOD) and the Race-Related Events Scale (RRES). The EOD consists of an 11-item experience of discrimination subscale and a 9-item major discrimination subscale [47]. The summary score for each subscale is the total number of situations where participants reported experiencing discrimination or receiving unfair treatment [47]. The RRES is a 23-item scale of yes-or-no questions that assess whether certain discriminatory situations have been experienced, such as “being treated rudely or coldly” [48]. The “yes” responses are summed to create a total score [48]. There is an additional open-ended item for participants to fill in situations not listed [48].
4.3.4. DNA Methylation Preprocessing
Participants provided saliva samples using Oragene-500 Format tubes at the first interview [49]. They were asked not to eat, drink, smoke, or chew gum for 30 min prior to providing the sample, and each participant spit into a tube repeatedly until the liquid reached a fill line of two milliliters (mL) [49]. Participants failing to fill the tube to the 2 mL line were given a clear lollipop to stimulate saliva production [49]. Each participant’s tube was then labeled with a barcode, which was entered into a freezer inventory; samples were then stored at 4 °C [49]. The Illumina Infinium Methylation EPIC (850 K) BeadChip was used to analyze epigenome-wide DNAm [49]. DNAm data were obtained through measurement of the fluorescent signals from methylated and unmethylated signals at each site; Intensity Data (IDAT) files were generated to store these measurements [49,50].
The raw IDAT files, along with the manifest file containing phenotype data, were imported into RStudio using the minfi package [51]. In DNAm studies, preprocessing plays a crucial role in ensuring the quality and reliability of the data [52]. The key preprocessing steps include, but are not limited to, the following: (1) probe filtering, (2) background correction, (3) color balance adjustment, (4) data normalization, (5) probe-type bias correction, and (6) batch effect removal [53].
In our initial quality control step, detection p-values were calculated using the minfi “detectionP” function. We excluded probes from further analyses if the probes had a detection p > 0.01 in more than 20% of the samples [54]. To improve the accuracy of downstream analysis, methylation data were further preprocessed using the minfi “preprocessFunnorm” function [55]. Specifically, functional normalization removes unwanted technical variation using control probes as surrogates [53] and has been shown to outperform several other normalization approaches [56]. The final methylation data included 654,407 probes. The methylation level at each CpG site was quantified as a beta-value, which ranges from 0 (indicating no methylation) to 1 (indicating complete methylation) [57].
4.3.5. Statistical Analysis
The primary outcome measure was the level of depressive symptoms, a variable derived from the BDI scores. Descriptive statistics such as mean and standard deviation for the continuous variables and frequency and percentage for the categorical variables were calculated for the sociodemographic characteristics. Participants with missing data in BDI items were excluded from the analysis.
Differential methylation analysis was performed to identify differentially methylated CpG sites and regions associated with the level of depressive symptoms. Several R packages, including limma, minfi, bumphunter, and MissMethyl were utilized for this analysis. The limma package is widely used for differential expression analysis, but it can be adapted for differential methylation analysis in combination with minfi [58]. The “lmFit” and” eBayes” limma functions were used to test for differential methylation. Differential analyses were conducted at both the region and probe levels. The function “bumphunter” from the minfi package was employed to identify differentially methylated regions (referred to as bumps) associated with depressive symptoms. Additionally, the “dmpFinder” function was utilized to identify differentially methylated positions (CpG sites). Gene-set enrichment analysis was performed using the “gometh” function from missMethyl, as well as the “annotateTranscripts” and “matchGenes” functions from bumphunter to gain insights into the biological significance of the affected genes identified. Analyses for this study were performed in RStudio with R version 4.2.2.
5. Conclusions
In the current study, we examined associations between depressive symptoms and DNAm among Black women in the InterGEN study. Black women are an understudied group in epigenomic research [49], and this study adds to the literature on differential methylation and depressive symptoms in this population. Differential methylation analysis identified six CpG sites and 25 differentially methylated regions associated with levels of depressive symptoms, and half of those regions were annotated to genes associated with neurological pathways, functions, diseases, or disorders. This suggests that there is a neurological component to depression [36], which should be considered by clinicians when treating individuals with depression. In addition, neurological pathways could possibly be targets for new drugs developed to treat depression. Further research is necessary to determine whether these findings can be replicated in a more diverse population or whether these findings are specific to Black women. Subsequent studies should also strive for consistency in sample types and depressive-symptom screening methods to eliminate variability due to the use of different methods.
Supplementary Materials
The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/ijms25147681/s1.
Author Contributions
Conceptualization, B.T.; methodology, B.T. and Y.Z.; software, B.T. and Y.Z.; validation, B.T. and Y.Z.; formal analysis, B.T. and Y.Z.; investigation, C.C. and J.Y.T.; resources, C.C. and J.Y.T.; data curation, C.C. and J.Y.T.; writing—original draft preparation, B.T.; writing—review and editing, B.T., Y.Z., N.B.P., S.P.-T., R.M.C. and J.Y.T.; supervision, R.M.C. and J.Y.T.; project administration, C.C. and J.Y.T.; funding acquisition, B.T., C.C. and J.Y.T. All authors have read and agreed to the published version of the manuscript.
Funding
This research was supported by the National Institutes of Health’s National Institute of Nursing Research under award number R01NR013520. Author B.T. was supported by the National Institutes of Health’s National Center for Advancing Translational Sciences under award number TL1TR001875.
Institutional Review Board Statement
This study was conducted in accordance with the Declaration of Helsinki and was approved by the Institutional Review Board of Columbia University (#AAAS9653).
Informed Consent Statement
Informed consent was obtained from all participants involved in this study.
Data Availability Statement
Data are available from the authors with a Data Use Agreement upon reasonable request.
Conflicts of Interest
The authors declare no conflicts of interest. The funders had no role in the design of the study; in the collection, analyses, or interpretation of data; in the writing of the manuscript; or in the decision to publish the results.
References
- Malhi, G.S.; Mann, J.J. Depression. Lancet 2018, 392, 2299–2312. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Uchida, S.; Yamagata, H.; Seki, T.; Watanabe, Y. Epigenetic mechanisms of major depression: Targeting neuronal plasticity. Psychiatry Clin. Neurosci. 2018, 72, 212–227. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Labaka, A.; Goñi-Balentziaga, O.; Lebeña, A.; Pérez-Tejada, J. Biological Sex Differences in Depression: A Systematic Review. Biol. Res. Nurs. 2018, 20, 383–392. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lee, B. National, State-Level, and County-Level Prevalence Estimates of Adults Aged ≥18 Years Self-Reporting a Lifetime Diagnosis of Depression—United States, 2020. MMWR Morb. Mortal. Wkly. Rep. 2023, 72, 644–650. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Spikes, T.; Higgins, M.; Lewis, T.; Dunbar, S. The Effect of Contextualized Racial and Gendered Stressors, Social Support, and Depression on Hypertension Illness Perceptions and Hypertension Medication Adherence in Young African American Women with Hypertension. J. Cardiovasc. Nurs. 2020, 35, 576–587. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Corcoran, J.; Marinescu, I.; Vogelsang, C.; Kim, J.C.; Morgan, S. Prevalence of depression in women with low income living in developed countries. Depress. Anxiety 2021, 38, 1046–1053. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gao, X.; Barcelona, V.; DeWan, A.; Prescott, L.; Crusto, C.; Sun, Y.V.; Taylor, J.Y. Depressive Symptoms and Blood Pressure in African American Women: A Secondary Analysis from the InterGEN Study. J. Cardiovasc. Nurs. 2022, 37, E89–E96. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Martin, C.L.; Ghastine, L.; Wegienka, G.; Wise, L.A.; Baird, D.D.; Vines, A.I. Early Life Disadvantage and the Risk of Depressive Symptoms among Young Black Women. J. Racial Ethn. Health Disparities 2024, 11, 1819–1828. [Google Scholar] [CrossRef] [Scilit]
- Bailey, R.K.; Mokonogho, J.; Kumar, A. Racial and ethnic differences in depression: Current perspectives. Neuropsychiatr. Dis. Treat. 2019, 15, 603–609. [Google Scholar] [CrossRef] [Scilit]
- Boulkrane, M.S.; Fedotova, J.; Kolodyaznaya, V.; Micale, V.; Drago, F.; van den Tol, A.J.; Baranenko, D. Vitamin D and Depression in Women: A Mini-review. Curr. Neuropharmacol. 2020, 18, 288–300. [Google Scholar] [CrossRef] [Scilit]
- Albert, K.M.; Newhouse, P.A. Estrogen, Stress, and Depression: Cognitive and Biological Interactions. Annu. Rev. Clin. Psychol. 2019, 15, 399–423. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sassarini, D.J. Depression in midlife women. Maturitas 2016, 94, 149–154. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jovanova, O.S.; Nedeljkovic, I.; Spieler, D.; Walker, R.M.; Liu, C.; Luciano, M.; Bressler, J.; Brody, J.; Drake, A.J.; Evans, K.L.; et al. DNA methylation signatures of depressive symptoms in middle-aged and elderly persons: Meta-analysis of multiethnic epigenome-wide studies. JAMA Psychiatry 2018, 75, 949–959. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Depression. World Health Organization. Published 13 September 2021. Available online: https://www.who.int/news-room/fact-sheets/detail/depression (accessed on 14 January 2023).
- Mayer, L.; Corrigan, P.W.; Eisheuer, D.; Oexle, N.; Rüsch, N. Attitudes towards disclosing a mental illness: Impact on quality of life and recovery. Soc. Psychiatry Psychiatr. Epidemiol. 2022, 57, 363–374. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Penner-Goeke, S.; Binder, E.B. Epigenetics and depression. Dialogues Clin. Neurosci. 2019, 21, 397–405. [Google Scholar] [CrossRef] [Scilit]
- de Mendoza, V.B.; Huang, Y.; Crusto, C.A.; Sun, Y.V.; Taylor, J.Y. Perceived Racial Discrimination and DNA Methylation among African American Women in the InterGEN Study. Biol. Res. Nurs. 2018, 20, 145–152. [Google Scholar] [CrossRef] [Scilit]
- Park, C.; Rosenblat, J.D.; Brietzke, E.; Pan, Z.; Lee, Y.; Cao, B.; Zuckerman, H.; Kalantarova, A.; McIntyre, R.S. Stress, epigenetics and depression: A systematic review. Neurosci. Biobehav. Rev. 2019, 102, 139–152. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, D.; Meng, L.; Pei, F.; Zheng, Y.; Leng, J. A review of DNA methylation in depression. J. Clin. Neurosci. Off. J. Neurosurg. Soc. Australas. 2017, 43, 39–46. [Google Scholar] [CrossRef] [Scilit]
- Li, M.; D’Arcy, C.; Li, X.; Zhang, T.; Joober, R.; Meng, X. What do DNA methylation studies tell us about depression? A systematic review. Transl. Psychiatry 2019, 9, 68. [Google Scholar] [CrossRef] [Scilit]
- Lin, E.; Tsai, S.J. Epigenetics and Depression: An Update. Psychiatry Investig. 2019, 16, 654–661. [Google Scholar] [CrossRef] [Scilit]
- Stelzer, G.; Rosen, N.; Plaschkes, I.; Zimmerman, S.; Twik, M.; Fishilevich, S.; Stein, T.I.; Nudel, R.; Lieder, I.; Mazor, Y.; et al. The GeneCards Suite: From Gene Data Mining to Disease Genome Sequence Analyses. Curr. Protoc. Bioinforma 2016, 54, 1.30.1–1.30.33. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Roy Chowdhury, S.; Mittal, R.; Yadav, R.; Guglany, V. Teaching NeuroImage: Glutaredoxin-5–Associated Variant Nonketotic Hyperglycinemia: A Treatable Mitochondrial Cytopathy. Neurology 2024, 102, e208105. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Llaurador-Coll, M.; Rios, S.; García-Gavilán, J.F.; Babio, N.; Vilella, E.; Salas-Salvadó, J. Plasma levels of neurology-related proteins are associated with cognitive performance in an older population with overweight/obesity and metabolic syndrome. GeroScience 2023, 45, 2457–2470. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Göteson, A.; Isgren, A.; Jonsson, L.; Sparding, T.; Smedler, E.; Pelanis, A.; Zetterberg, H.; Jakobsson, J.; Pålsson, E.; Holmen-Larsson, J.; et al. Cerebrospinal fluid proteomics targeted for central nervous system processes in bipolar disorder. Mol. Psychiatry 2021, 26, 7446–7453. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Qiu, B.; Matthay, K.K. Advancing therapy for neuroblastoma. Nat. Rev. Clin. Oncol. 2022, 19, 515–533. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yahya, V.; Spagnolo, F.; Di Maggio, G.; Leopizzi, E.; De Marco, P.; Fortunato, F.; Comi, G.P.; Rini, A.; Monfrini, E.; Di Fonzo, A. Juvenile-onset dystonia with spasticity in Leigh syndrome caused by a novel NDUFA10 variant. Park. Relat. Disord. 2022, 104, 85–87. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sharma, L.K.; Lu, J.; Bai, Y. Mitochondrial respiratory complex I: Structure, function and implication in human diseases. Curr. Med. Chem. 2009, 16, 1266–1277. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Forsythe, E.; Kenny, J.; Bacchelli, C.; Beales, P.L. Managing Bardet–Biedl Syndrome—Now and in the Future. Front. Pediatr. 2018, 6, 23. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- N Syndrome. Orphanet. Published 10 April 2024. Available online: https://www.orpha.net/en/disease/detail/2608 (accessed on 28 April 2024).
- Zhang, M.; Wang, H. Ca2+-stimulated ADCY1 and ADCY8 regulate distinct aspects of synaptic and cognitive flexibility. Front. Cell Neurosci. 2023, 17, 1215255. [Google Scholar] [CrossRef] [Scilit]
- Li, H.; Yu, S.; Wang, R.; Sun, Z.; Zhou, X.; Zheng, L.; Yin, Z.; Zhang, X.; Sun, Y. ARHGEF10 gene polymorphism is closely associated with the risk of ischemic stroke in Northern Han Chinese population. Neurol. Res. 2017, 39, 158–164. [Google Scholar] [CrossRef] [Scilit]
- Huang, S.; Zheng, C.; Xie, G.; Song, Z.; Wang, P.; Bai, Y.; Chen, D.; Zhang, Y.; Lv, P.; Liang, W.; et al. FAM19A5/TAFA5, a novel neurokine, plays a crucial role in depressive-like and spatial memory-related behaviors in mice. Mol. Psychiatry 2021, 26, 2363–2379. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zheng, D.; Liu, X. Cochlear Implantation Outcomes in Patients with OTOF Mutations. Front. Neurosci. 2020, 14, 447. [Google Scholar] [CrossRef] [Scilit]
- Miyake, C.Y.; Burrage, L.; Glinton, K.; Houck, K.; Hoyos-Martinez, A.; Graham, B.; Yang, Y.; Rawls-Castillo, B.; Scaglia, F.; Soler-Alfonso, C.; et al. TANGO2 Deficiency. In GeneReviews®; Adam, M.P., Feldman, J., Mirzaa, G.M., Pagon, R.A., Wallace, S.E., Bean, L.J.H., Gripp, K.W., Amemiya, A., Eds.; University of Washington: Seattle, WA, USA, 1993. Available online: http://www.ncbi.nlm.nih.gov/books/NBK476443/ (accessed on 3 May 2024).
- Li, S.; Wen, B.; Zhao, W.; Wang, L.; Chen, X. Design, Synthesis and Biological Evaluation of Novel Ketamine Derivatives as NMDAR Antagonists. Molecules 2024, 29, 2459. [Google Scholar] [CrossRef] [Scilit]
- Kabotyanski, K.E.; Najera, R.A.; Banks, G.P.; Sharma, H.; Provenza, N.R.; Hayden, B.Y.; Mathew, S.J.; Sheth, S.A. Cost-effectiveness and threshold analysis of deep brain stimulation vs. treatment-as-usual for treatment-resistant depression. Transl. Psychiatry 2024, 14, 243. [Google Scholar] [CrossRef] [Scilit]
- Kanner, A.M. Is major depression a neurologic disorder with psychiatric symptoms? Epilepsy Behav. 2004, 5, 636–644. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jüllig, A.K.; Hebib, S.; Metzker, H.; Gruber, E.; Gruber, O. Task-induced deactivation dysfunction during reward processing is associated with low self-esteem in a possible subtype of major depression. Brain Behav. 2024, 14, e3545. [Google Scholar] [CrossRef] [Scilit]
- Poletti, S.; Mazza, M.G.; Benedetti, F. Inflammatory mediators in major depression and bipolar disorder. Transl. Psychiatry 2024, 14, 247. [Google Scholar] [CrossRef] [Scilit]
- Ma, F.; Bian, H.; Jiao, W.; Zhang, N. Single-cell RNA-seq reveals the role of YAP1 in prefrontal cortex microglia in depression. BMC Neurol. 2024, 24, 191. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Choi, S.W.; Schalet, B.; Cook, K.F.; Cella, D. Establishing a common metric for depressive symptoms: Linking the BDI-II, CES-D, and PHQ-9 to PROMIS depression. Psychol. Assess. 2014, 26, 513–527. [Google Scholar] [CrossRef] [Scilit]
- Maki, K.A.; DeVon, H.A. A nursing theory-guided framework for genetic and epigenetic research. Nurs. Inq. 2018, 25, e12238. [Google Scholar] [CrossRef] [Scilit]
- Crusto, C.A.; Barcelona de Mendoza, V.; Connell, C.M.; Sun, Y.V.; Taylor, J.Y. The Intergenerational Impact of Genetic and Psychological Factors on Blood Pressure Study (InterGEN): Design and Methods for Recruitment and Psychological Measures. Nurs. Res. 2016, 65, 331–338. [Google Scholar] [CrossRef] [Scilit]
- Beck, A.T.; Ward, C.H.; Mendelson, M.; Mock, J.; Erbaugh, J. An Inventory for Measuring Depression. Arch. Gen. Psychiatry 1961, 4, 561–571. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Beck, A.T.; Steer, R.A.; Carbin, M.G. Psychometric properties of the Beck Depression Inventory: Twenty-five years of evaluation. Clin. Psychol. Rev. 1988, 8, 77–100. [Google Scholar] [CrossRef] [Scilit]
- Krieger, N.; Smith, K.; Naishadham, D.; Hartman, C.; Barbeau, E.M. Experiences of discrimination: Validity and reliability of a self-report measure for population health research on racism and health. Soc. Sci. Med. 1982 2005, 61, 1576–1596. [Google Scholar] [CrossRef] [Scilit]
- Waelde, L.C.; Pennington, D.; Mahan, C.; Mahan, R.; Kabour, M.; Marquett, R. Psychometric properties of the Race-Related Events Scale. Psychol. Trauma Theory Res. Pract. Policy 2010, 2, 4–11. [Google Scholar] [CrossRef] [Scilit]
- Taylor, J.Y.; Wright, M.L.; Crusto, C.A.; Sun, Y.V. The Intergenerational Impact of Genetic and Psychological Factors on Blood Pressure (InterGEN) Study: Design and Methods for Complex DNA Analysis. Biol. Res. Nurs. 2016, 18, 521–530. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Smith, M.L.; Baggerly, K.A.; Bengtsson, H.; Ritchie, M.E.; Hansen, K.D. illuminaio: An open source IDAT parsing tool for Illumina microarrays. F1000Research 2013, 2, 264. [Google Scholar] [CrossRef] [Scilit]
- Aryee, M.J.; Jaffe, A.E.; Corrada-Bravo, H.; Ladd-Acosta, C.; Feinberg, A.P.; Hansen, K.D.; Irizarry, R.A. Minfi: A flexible and comprehensive Bioconductor package for the analysis of Infinium DNA methylation microarrays. Bioinforma 2014, 30, 1363–1369. [Google Scholar] [CrossRef] [Scilit]
- Ori, A.P.S.; Lu, A.T.; Horvath, S.; Ophoff, R.A. Significant variation in the performance of DNA methylation predictors across data preprocessing and normalization strategies. Genome Biol. 2022, 23, 225. [Google Scholar] [CrossRef] [Scilit]
- Feil, D.; Abrishamcar, S.; Christensen, G.M.; Vanker, A.; Koen, N.; Kilanowski, A.; Hoffman, N.; Wedderburn, C.J.; Donald, K.A.; Kobor, M.S.; et al. DNA methylation as a potential mediator of the association between indoor air pollution and neurodevelopmental delay in a South African birth cohort. Clin. Epigenetics 2023, 15, 31. [Google Scholar] [CrossRef] [Scilit]
- Heiss, J.A.; Just, A.C. Improved filtering of DNA methylation microarray data by detection p values and its impact on downstream analyses. Clin. Epigenetics 2019, 11, 15. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fortin, J.P.; Triche, T.J.; Hansen, K.D. Preprocessing, normalization and integration of the Illumina HumanMethylationEPIC array with minfi. Bioinformatics 2017, 33, 558–560. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fortin, J.P.; Labbe, A.; Lemire, M.; Zanke, B.W.; Hudson, T.J.; Fertig, E.J.; Greenwood, C.M.; Hansen, K.D. Functional normalization of 450k methylation array data improves replication in large cancer studies. Genome Biol. 2014, 15, 503. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xie, C.; Leung, Y.K.; Chen, A.; Long, D.X.; Hoyo, C.; Ho, S.M. Differential methylation values in differential methylation analysis. Bioinforma 2019, 35, 1094–1097. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ritchie, M.E.; Phipson, B.; Wu, D.; Hu, Y.; Law, C.W.; Shi, W.; Smyth, G.K. Limma powers differential expression analyses for RNA-sequencing and microarray studies. Nucleic Acids Res. 2015, 43, e47. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2024 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).