


Simple Summary
The Baird’s tapir (Tapirus bairdii) is the largest terrestrial mammal in Mesoamerica. It plays an important ecological role in maintaining diverse tropical forests through seed dispersal in its faeces. However, knowledge about the composition of its diet remains scattered. This review revealed that the Baird’s tapir consumes just over 500 plant taxa in the different ecosystems it inhabits. Its diet consists mainly of stems, leaves, fruits, bark, and flowers. The influence of seasonality on the tapir’s diet is unclear due to the underestimation (fruits) and overestimation (fibre) of some components. We have identified limitations in the techniques used to determine diet components and study designs. This review offers insights that could inform future studies aiming to elucidate the direct and indirect effects of Baird’s tapirs on vegetation in their habitat and their influence on ecosystem dynamics.
Abstract
Baird’s tapir (Tapirus bairdii) plays an important ecological role in Mesoamerican forests as a browser and seed disperser, earning it the nickname of “gardener of the forest”. However, knowledge of its diet composition remains scattered. We reviewed and analysed the available literature on the composition of Baird’s tapir diet throughout its geographic distribution, compiling data from 27 studies. Baird’s tapir was found to consume 515 plant taxa belonging to 410 genera and 123 families. Five types of dietary components have been identified: fibre (stems), leaves, fruit, bark, and flowers. The influence of seasonality on the tapir diet is unclear due to the underestimation of some components, notably fruits. We identified limitations in the techniques used to determine diet components and study designs. Future research should focus on developing techniques to improve the quantification of dietary components. Additionally, the direct and indirect effects of the Baird’s tapir’s diet and plant consumption on ecosystem dynamics should be investigated to clearly understand the functional role of this species.
1. Introduction
Large wild herbivores play a critical role in determining the structure and function of ecosystems [1], although some of their direct and indirect trophic relationships with plants, small vertebrates, invertebrates, and predators remain unknown [2,3]. To understand the effects of these organisms on plant diversity and vegetation dynamics, it is necessary to investigate their feeding habits and strategies, the components of their diet, the return of nutrients through excreta, and the mechanical impacts on soil and plants [2,4,5]. The diet composition of herbivores is particularly useful to understand habitat preference, plant selection, animal movements, health, evolution, and trophic ecology [6,7,8,9,10,11,12,13].
The diet of an herbivore can be defined as the range of plants it consumes. These plants are chosen based on their availability, as well as the metabolic needs and the anatomy of the digestive tract of herbivores [14]. A comprehensive understanding of the composition of herbivores’ diets and their staple foods is crucial, as these are fundamental to their life cycle strategy (e.g., growth, reproduction, fitness, survival) [15,16] and for their conservation.
At present, large herbivores are facing many anthropogenic threats that can reduce food availability or quality. These include competition with livestock, land use change, climate change, and invasive species [17]. In this scenario, the populations of these species could decline due to several factors, including the limited availability of high-quality food, energy depletion from increased foraging, and malnutrition, leading to low reproduction or decreased survival [18].
Among the large herbivore species that are facing anthropogenic threats are the four extant species of the Tapiridae family. These threats jeopardise their ecological role as seed dispersers, which contributes to forest regeneration and maintenance as well as landscape connectivity and diversity [19,20]. Tapirs are distributed across North and Central America (Tapirus bairdii), South America (T. bairdii, Tapirus pinchaque, and Tapirus terrestris), and Southeast Asia (Tapirus indicus) [21]. They inhabit a wide variety of vegetation types, including dry to evergreen tropical forests, montane forests, shrub forests, grasslands, and xeric formations [21,22,23]. Consequently, their diet includes a huge diversity of species.
The Baird’s tapir (T. bairdii) is known as the ‘gardener’ of Mesoamerican forests [24]. The species is distributed from southeastern Mexico to northwestern Colombia [25], where it inhabits areas that are global hotspots of biodiversity, home to around 24,000 plant species [26,27]. Baird’s tapir home range varies between 1 and 24 km2, moving up to 3 km per day [28,29]. These movements enable them to use different types of vegetation with varying degrees of disturbance and interact with many species [30,31]. How Baird’s tapir shapes its environment through its influence on vegetation and nutrient cycling is less clear, despite being one of the most studied species in this field. In particular, the available information is scattered, making it difficult to understand its role in the different ecosystems it inhabits.
This study contributes to the basic understanding of the functional role of Baird’s tapir by reviewing the locations where research on the species has been conducted, the plant species and parts it consumes, and the methods used to determine its diet and quantify its components. The study also addresses the influence of seasonality on Baird’s tapir diet. The results may guide future research into techniques that improve the standardisation of the identification and quantification of dietary components. This will provide the robust foundation necessary to understand the role of tapirs in shaping their environment.
2. Materials and Methods
We carried out a comprehensive review of the existing literature on the diet of T. bairdii using six search engines: Google Scholar, Red de Revistas Científicas de America Latina y el Caribe, España y Portugal (Redalyc project), Science Direct, Science Electronic Library Online (Scielo), Scopus, and Web of Knowledge. We conducted the search both in English and Spanish. A systematic search was temporally delimited from 1978 to 2024, using the following combinations: “Tapir” + “Baird” + “Diet” and, in Spanish, “dieta” + “tapir” + “Baird”. We included all contributions in scientific journals (articles and scientific notes), newsletters of the IUCN Tapir Specialists Group, abstracts from conferences and workshops, reports, and theses. Studies conducted with the same data were considered as one; they included Tobler [32] and Tobler et al. [33], as well as Foerster [34] and Foerster and Vaughan [35]. Contributions without original data were excluded.
We built a database on studies on the diet of Baird’s tapir in Microsoft 365 Excel (version 16.105.1) with the following information: publication details (title, authors, year of publication, and year of sampling), country, region, sampling location coordinates, season, sample size, technique used to identify plant species consumed, technique used to quantify diet components, and percentage of diet components. Separately, we built another database in Excel containing the family, genus, and species of plants consumed by the Baird’s tapir; the location and country where the study was carried out; and publication details such as authors and year of publication.
A correspondence analysis was used to explore the relationships among vegetation types used by Baird’s tapirs and the plant species they consume. This analysis allows us to show the relative positions among variables, hence their relationships, where shorter distances indicate higher relationships and associations [36]. The analysis was performed using R 4.5.2 [37].
3. Results
3.1. Locations
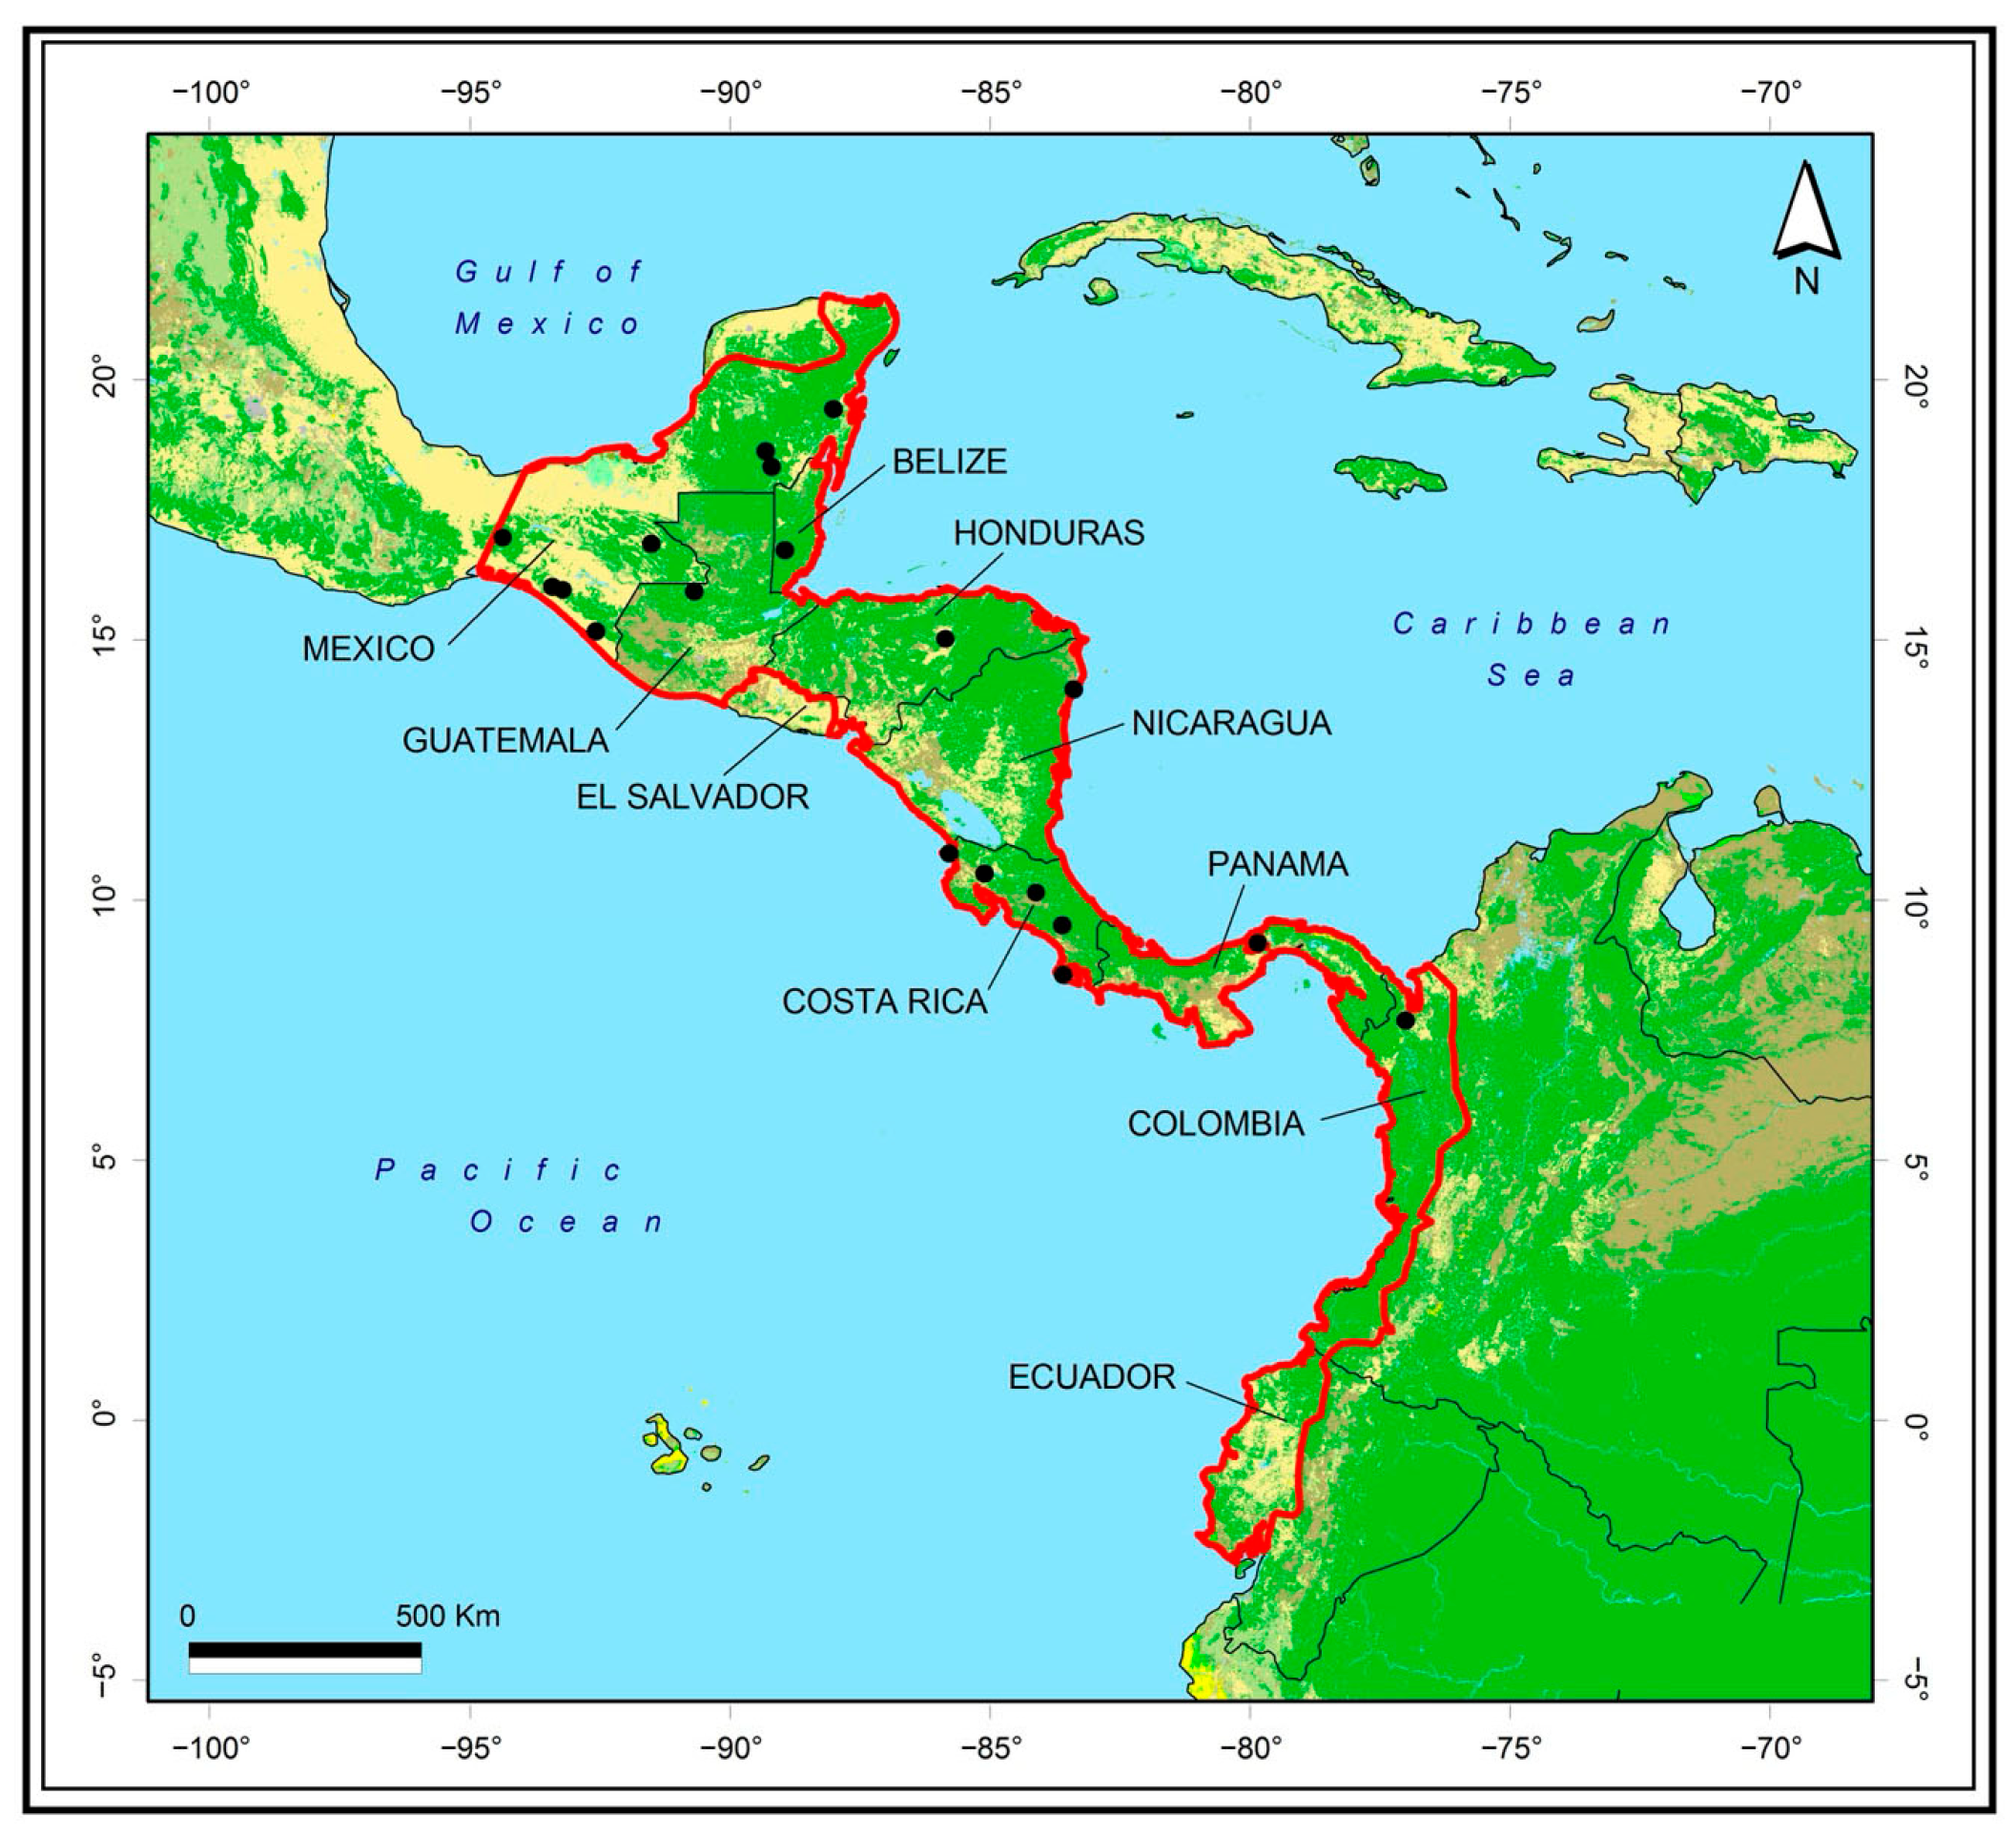
We found 27 studies related to the diet composition of T. bairdii from seven countries (Figure 1). Mexico and Costa Rica are the countries with the highest number of studies (13 and 6, respectively), followed by Colombia and Panama (2 each), and the other countries (Belize, Guatemala, Honduras, and Nicaragua) with one study each (Supplementary Table S1 [24,32,33,34,35,38,39,40,41,42,43,44,45,46,47,48,49,50,51,52,53,54,55,56,57,58,59,60,61]).
Figure 1.
Map showing the geographic distribution of Tapirus bairdii (red area). The black dots represent the sites where studies about diet composition have been carried out.
3.2. Techniques Used to Identify Plant Species Consumed
The plant species consumed by Baird’s tapirs were identified by browsing signs, faecal analysis, direct observations (by observers or camera traps), and interviews with local people. The most used techniques in the studies were the combination of browsing signs and faecal analysis (10 out of 20 studies; Table 1).
Table 1.
Studies with reports on plants consumed by Baird’s tapir in its geographic range. B = browse, F = faeces, B/F = browse and faeces, and O = others (interviews with local people, review). X indicates the use of a given identification technique in a given study; - indicates it was not used.
3.3. Plant Species Consumed
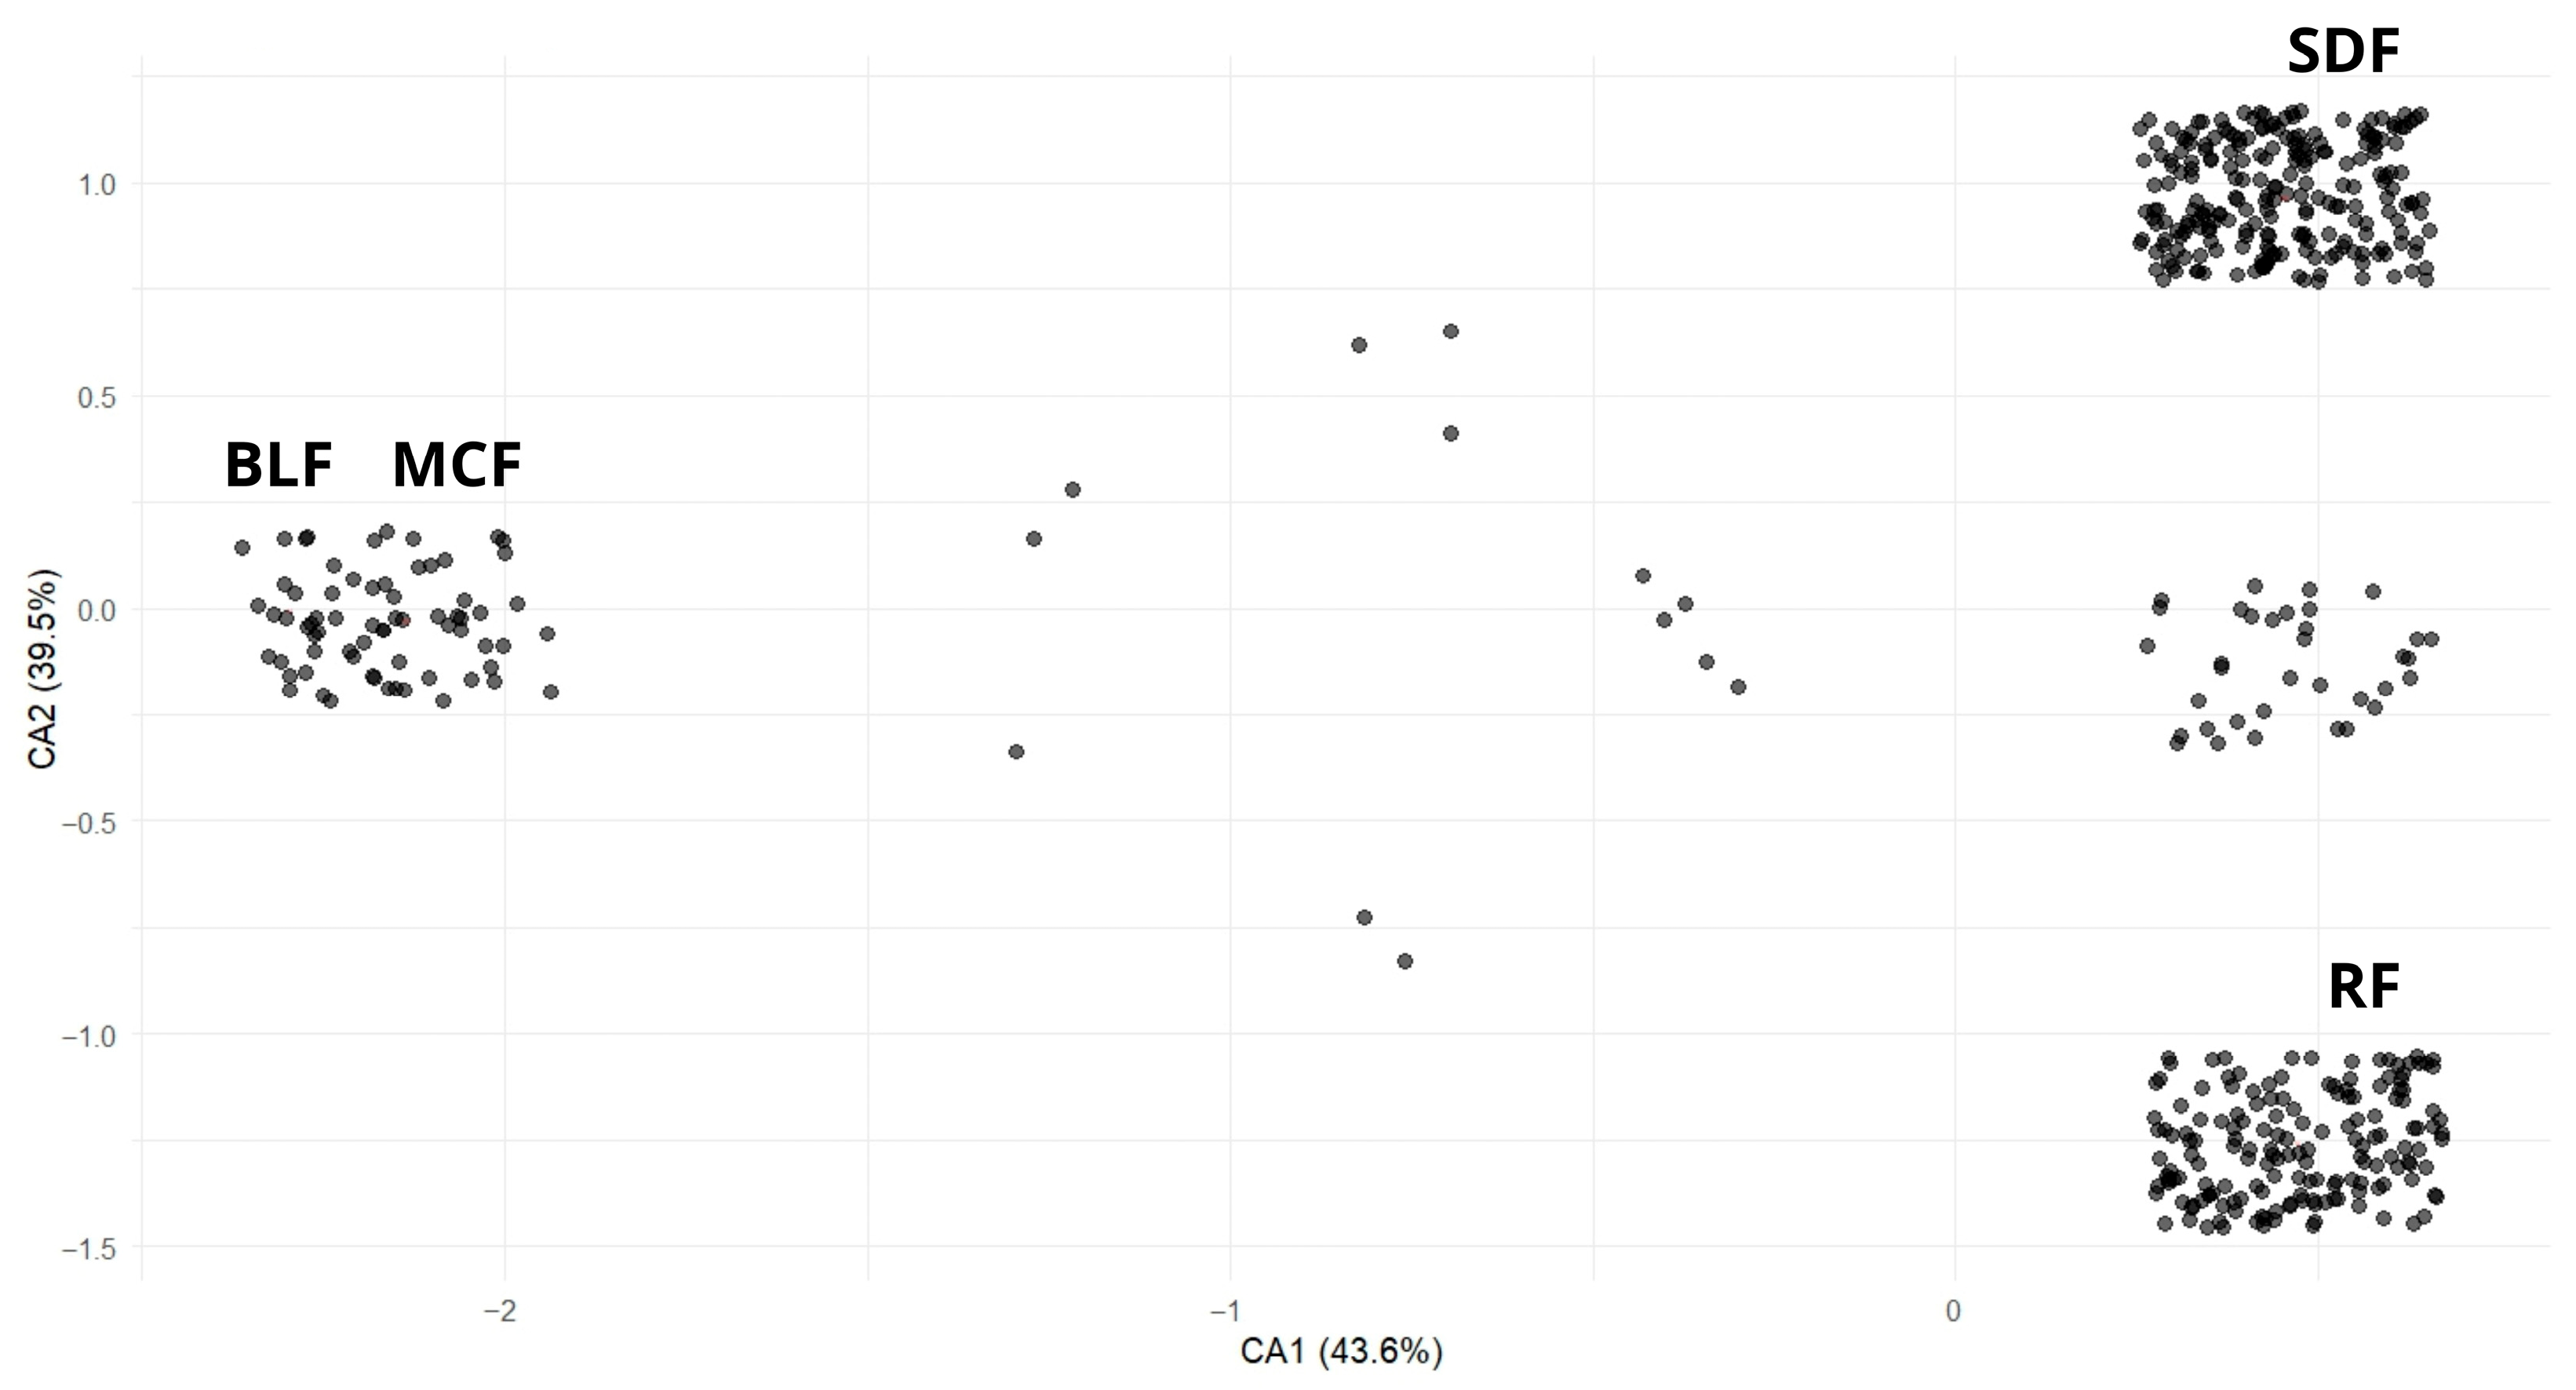
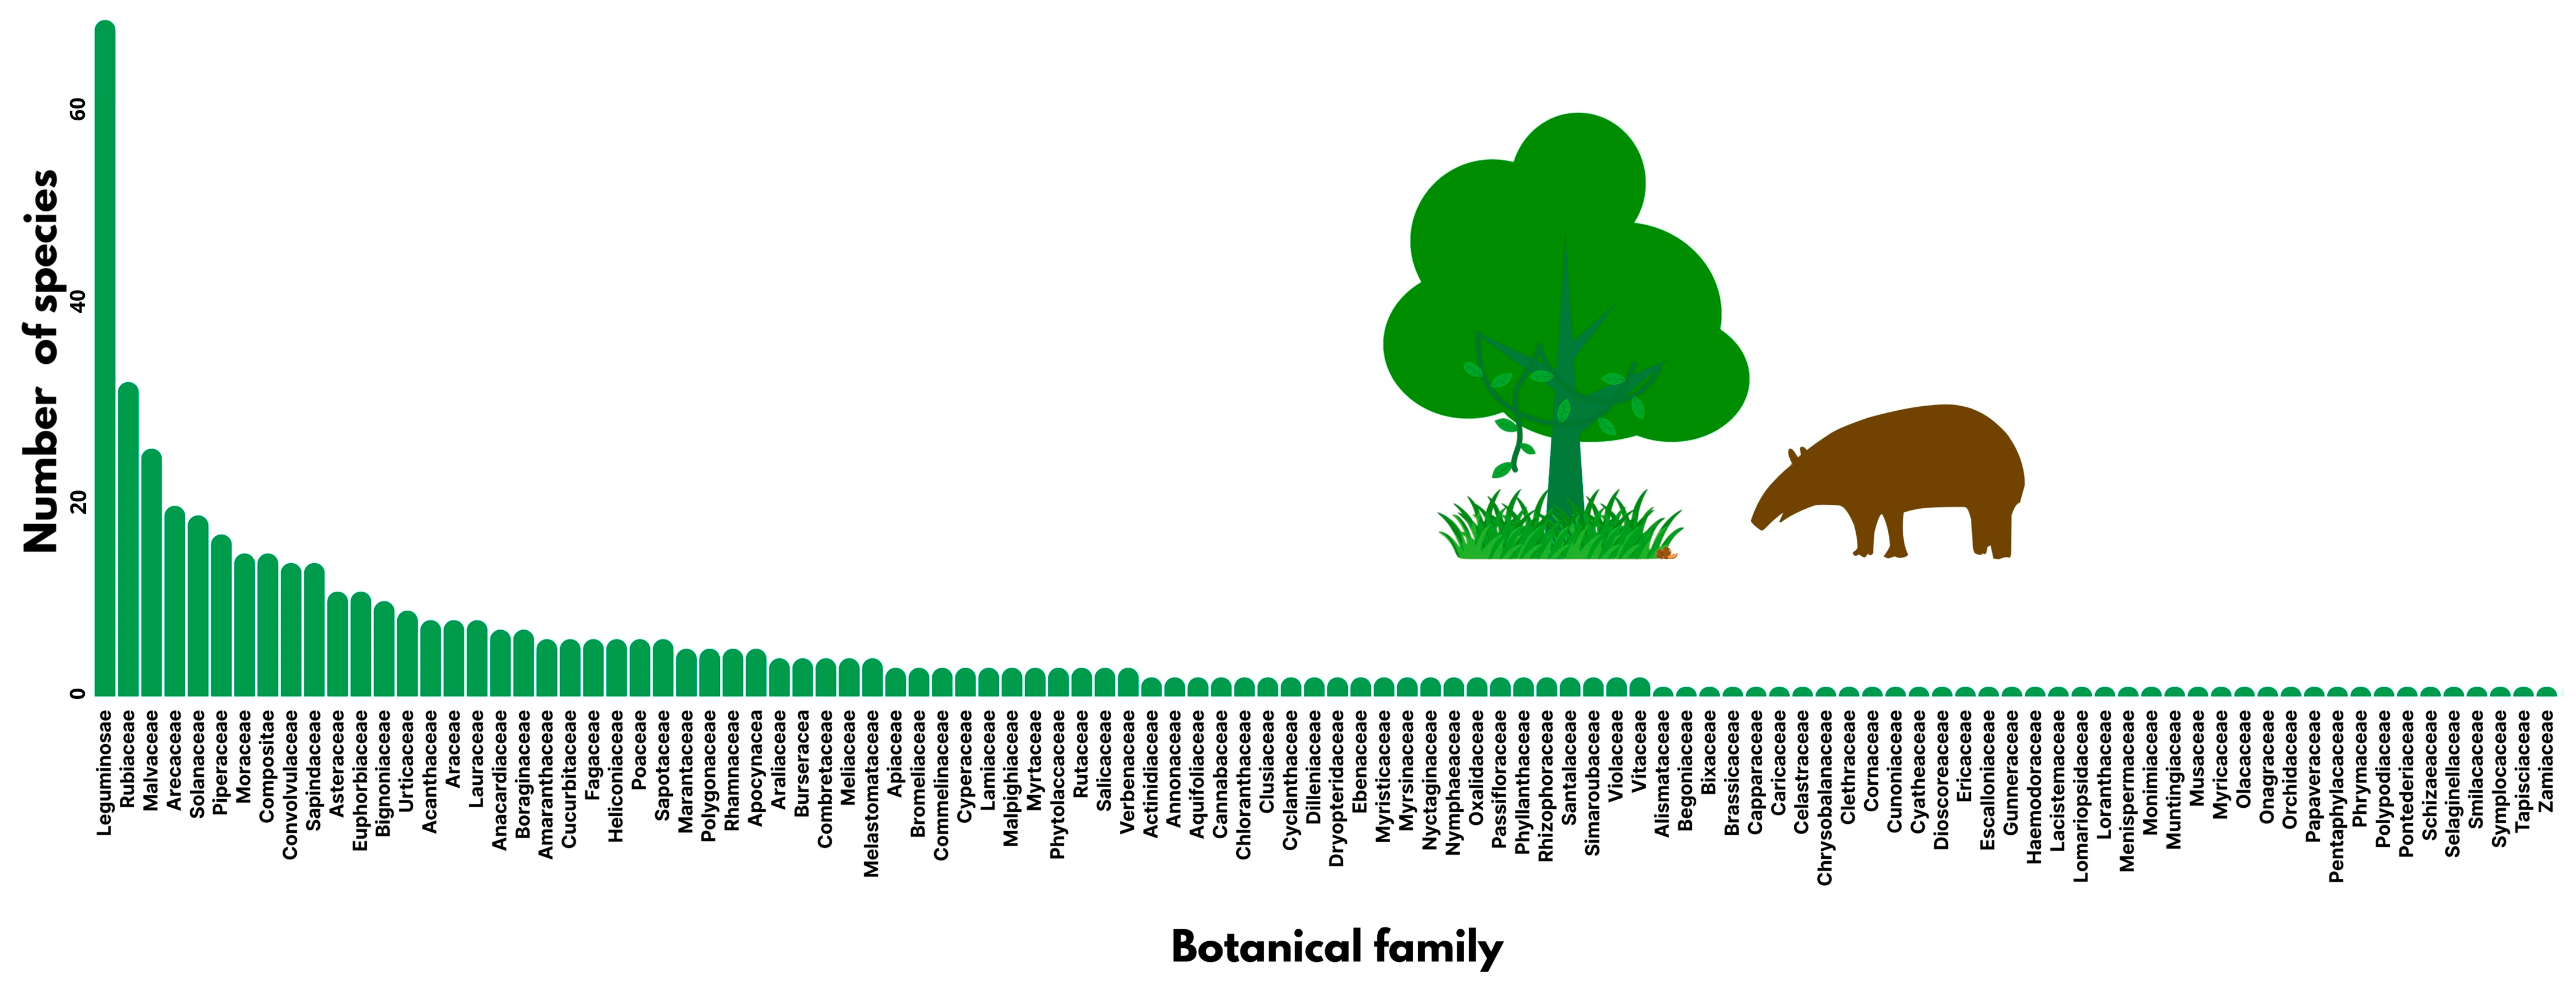
The studies were carried out in four types of tropical forest: broadleaf forest (BLF; 1 study), mountain cloud forest (MCF; 6 studies), semideciduous forest (SDF; 9 studies), and rainforest (RF; 11 studies). They encompassed 515 species of plants consumed by T. bairdii, belonging to 410 genera and 123 families (Supplementary Table S2 [38,39,40,41,42,43,44,45,46,47,48,49,50,51,52,53,54,55,56,57,58,59,60,61]). Although most species consumed by tapirs were specific to one type of tropical forest, five species were associated with three types of forest. Aphelandra schiedeana, Ficus insipida, and Spondias mombin were associated with MCF, SDF, and RF. Piper auritum and Cecropia peltata were associated with MCF, BLF, and SDF (Figure 2). The four most frequently documented plant species were Brosimum alicastrum and S. mombin (8 studies), Manilkara zapota (7), and Acalypha diversifolia (6). Genera with the highest number of species were Piper (17), Psychotria (13), Solanum (10), and Ipomoea (8). Families with the highest number of species were Leguminosae (71 species), Rubiaceae (33), Malvaceae (26), Arecaceae (20), and Solenaceae (19) (Figure 3).
Figure 2.
The correspondence analysis indicates that Tapirus bairdii consumes plant species that are specific to each type of tropical forest, except for BLF and MCF. BLF = broadleaf forest; MCF = mountain cloud forest; SDF = semideciduous forest; RF = rainforest. To prevent overplotting, geom_jitter was used in ggplot.
Figure 3.
Number of species per family of plants consumed by Tapirus bairdii. Families in which only the genus was found were excluded from the graphic.
3.4. Techniques Used to Quantify Diet Components
Three methods have been utilised to quantify the components of the Baird’s tapir’s diet, two based on faecal matter and one on direct observation of foraging activity. The faecal-based methods used are frequency by occurrence (9 studies) and weight of each component (7), although five studies have combined both methods. Direct observation of foraging activity has only been used in one study. For this study, observers recorded the parts of plants eaten by the tapir (leaves, fruits, bark, stems, or flowers) at five-minute intervals for periods ranging from two to 11 h over almost one year [35].
3.5. Diet Composition
Five dietary components have been recorded: bark, fibre or stems (parts of plants with a diameter > 1 mm), flowers, fruits, and leaves, of which the most frequently mentioned are fibre or stems, leaves, and fruits (13 studies), while bark and flowers are mentioned less frequently (2 and 1 studies, respectively).
Studies were carried out in four types of forest (Table 2 and Table 3) over periods of between 4 and 24 months (Table 2 and Table 3). As a result, dietary components varied widely among studies, even in the same type of vegetation. Moreover, they should not be interpreted as equivalent due to the different methodologies used to quantify them. In studies based on the frequency per occurrence method, fibre represented 7.6–68.0%, leaves 18.6–65.4%, and fruits 0.3–27.2% (Table 2). Using the component weighing method, the percentages were: fibre 11.9–43.6%, leaves 41.1–79.7%, fruits 2.2–47%, and bark 2% (Table 3). The percentages from direct observations (one study only) were, in decreasing order of importance, leaves 67%, fruits 19%, fibre 12%, bark 2%, and flowers 0.1% [35]. Note that the study by Mejía-Correa et al. [40] was omitted because the researchers summed the percentages of fibre and leaves (a total of 83%), making it impossible to determine the percentage of each component.
Table 2.
Studies quantifying the components of the Baird’s tapir’s diet using the frequency per occurrence technique. The studies are listed in increasing order of samples analysed. Asterisks (*) indicate studies that also used the frequency per occurrence technique. MCF = mountain cloud forest; SDF = semideciduous forest; RF = rainforest.
Table 3.
Diet component percentages in studies analysing the Baird’s tapir’s diet using the weighing technique. Studies are organised in increasing order of sample size. BLF = Broadleaf Forest; MCF = mountain cloud forest; SDF = semideciduous forest; RF = rainforest.
3.6. Influence of Seasonality on Diet
Five studies compared the dietary composition between dry and rainy seasons by analysing the frequency of occurrence in faeces (Table 4). Of these, four were conducted in Mexico (in three vegetation types: MCF, RF, and SDF) and one in Costa Rica (in RF). All the studies reported that leaves are more frequent during the rainy season, while four reported more fibre in the dry season, and three reported more fruits in the dry season. Six studies compared diet seasonal variation with the component weighting method (Table 5). Four of these studies were conducted in Mexico (in MCF, RF, and SDF), with the remainder carried out in Costa Rica (RF) and Guatemala (RF). In four studies, leaves represented a higher percentage during the rainy season, while in three studies, fibre represented a higher percentage in the rainy season, whereas the three others found the contrary, and four reported a higher percentage of fruit in the dry season.
Table 4.
Studies analysing the influence of seasonality (dry and rainy seasons) on the components of Baird’s tapir diet using the frequency per occurrence technique. D = dry season; R = rainy season.
Table 5.
Studies analysing the influence of seasonality (dry and rainy seasons) on the components of Baird’s tapir diet using the weighing technique. D = dry season; R = rainy season.
The only study using direct observation to investigate tapir feeding revealed that during the dry season, the percentage of leaves (68.1%), fibre (18.8%), and flowers (0.3%) in the diet was higher than during the rainy season (leaves 66.9%; fibre 7.9%; flowers 0%) [35]. However, the percentage of fruit and bark was higher in the rainy season than in the dry season (fruit 22.3% and 12.4%, bark 3% and 0.4%, respectively).
4. Discussion
This review aimed at compiling the available information on Baird’s tapir diet, including study locations, the plant species and parts consumed, the methods used to determine its diet and quantify its components, and the influence of seasonality on its diet. The results revealed geographic gaps within Baird’s tapir distribution range where its diet has not been studied. This review also provides a current list of plant species forming part of the tapir’s diet, which is the most extensive to date, surpassing the previous estimate of 100 to 150 species by Foerster and Vaughan [34]. Our review also indicates that the remnants detected in Baird’s tapir faeces could be misleading indicators of dietary composition if they are assumed to reflect the quantity of each dietary component. Seasonality appears to have little influence on the tapir’s diet, potentially because the techniques employed do not accurately quantify its components, with some highly digestible components, such as fruits, being likely underestimated. Our results underscore the need to implement more efficient techniques to understand basic but very important aspects of the feeding ecology of the Baird’s tapir.
4.1. Techniques Used to Identify Plant Species Consumed
The analysis of faecal residues and the observation of browsing signs and direct foraging activity remain proven effective techniques, but future research could incorporate molecular analyses to identify plant tissue DNA directly from faeces, as well as interviews with local experts, camera trap monitoring, and stable isotope analyses [62,63,64]. For instance, combined genetic and ethnobotanical approaches in Hibert et al.’s [63] study revealed new species, genera, and families in the lowland tapir’s diet in French Guiana.
Traditional techniques such as the microhistological analysis of faecal remains and the identification of browsing signs remain widely used to this day. These two techniques are low-cost. In the first case, students typically carry out the entire procedure, which keeps the labour costs quite low. However, one disadvantage is that a collection of all the plants found in the tapir’s habitat is necessary for comparison with the plants found in the faeces. In the case of browsing signs, labour costs are also low. However, it requires extensive experience in tracking these animals, a skill that researchers and students might not possess. An experienced local guide is therefore an asset, but this raises the costs.
The use of DNA metabarcoding to identify the plant species consumed by tapirs has recently proved to be a very useful technique. It has been possible to identify a high percentage of plants at the family level (95.1%) and genus level (74.4%) by studying highly degraded plant fragments found in faeces. While this technique is regarded as cost-effective [65], it remains costly in certain regions and for academic groups with limited financial resources [66]. This may be the reason why only one study using DNA metabarcoding has been conducted on tapirs to date, in a rich country [2]. Furthermore, it should be noted that taxonomic resolution is a significant limitation of this approach, which often provides results at the family or genus level only when sequences are similar or because the reference databases are not complete [2].
4.2. Techniques Used to Quantify Diet Components
The analysis of faeces has been used to assess the dietary composition and diversity, dietary patterns, and feeding behaviour of a wide variety of wild species (see [67]). Several studies have sought to quantify the components of the Baird’s tapir diet by analysing faecal remnants [39,43,48]. However, the technique in which the components (fruits, bark, leaves) are separated, oven-dried, and quantified in relation to the initial sample volume [68,69] does not appear to be suitable for achieving this objective. Techniques using post-ingestive samples are subject to several factors that affect the accuracy and precision of diet estimation [70]. For example, different digestion rates and the greater fragmentation and decomposition of softer components (e.g., pulp and young leaves) compared to harder components (e.g., stems and seeds) will change the estimation of the dietary components [70]. Only one study has used direct observation of feeding animals to determine the dietary components of Baird’s tapirs [35]. This technique has been widely used to observe the food preferences of wild animals [71], although it has been in disuse over the years [70]. It is notably difficult to employ in areas where there is limited visual range, such as in forests, and it is time-consuming. Although this technique allows gathering quantitative data and has limitations in the accuracy of quantifying and separating certain components, such as fibre.
4.3. Plant Species Consumed
The current list of plant species forming part of the Baird’s tapir diet provided by this review surpasses the estimations of 100–150 species by Foerster and Vaughan [35] and those of both the lowland tapir (T. terrestris) (460 species; [72]), and the Malayan tapir (T. indicus) (380 species; [73]). With 515 identified plant species, the Baird’s tapir diet appears the most diverse among its genus, although this number could increase, as studies to date have been limited mainly to two countries (Mexico and Costa Rica), with some missing parts of its geographic range (Mesoamerica), where an estimated 20,000 plant species exist [74]. The diversity of the Baird’s tapir diet may be related to the wide variety of habitats and vegetation types in which it lives, including marshes, mangroves, swamps, tropical rainforests, riparian forests, monsoon deciduous forests, dry deciduous forests, and montane cloud forests [75,76]. Consequently, the potential influence of Baird’s tapir on the ecosystems and landscapes it inhabits could be greater than previously thought, given the large number of plants with which it interacts.
Due to the wide variety of plant species they consume, tapirs are considered generalist herbivores. The differences in diet among different studies can be attributed primarily to the characteristics of the habitat [77]. This finding aligns with the results of the correspondence analysis, which revealed that tapirs consume species characteristic of each vegetation type they inhabit, with only a few species shared between them. Some of the species shared, such as S. mombin, C. peltata, and F. insipida, are important due to their fruit, which is important to numerous wildlife species (birds, bats, monkeys, coatis, and deer; [78,79]). The leaves of P. auritum and C. peltata are a food source for animals, while A. schiedeana is of significant interest due to its flowers, which attract pollinating species.
4.4. Diet Composition
The natural diet of tapirs has been described as predominantly resulting from browsing, with a low percentage of fruit [80]. The results from this review support this view, with most studies (except [39]) reporting percentages of fruits that do not exceed 10%, the balance being fibre and leaves. We should be aware that the quantity of fruits consumed by tapirs has been estimated by counting or weighing the seeds, skin remnants, and pulp found in their faeces, leading to biassed estimations.
Although tapirs are estimated to have a low fruit consumption, their ecological impact on fruit seed dispersal may be quite high, as they can disperse almost 10,000 seeds per ha/year [20]. Furthermore, thanks to their large size, long intestinal retention times, and wide distribution areas, they can disperse seeds of different sizes and over greater distances [19]. Additionally, recent studies have found that seeds defecated by tapirs have a higher germinability and accelerated germination time compared to manually depulped seeds [81]. This contributes to forest regeneration and helps maintain critical ecosystem functions, such as the maintenance of forest carbon stocks [82].
4.5. Influence of Seasonality on Diet
One of the main limitations in determining whether seasonality influences the diet of Baird’s tapirs is that the vast majority of studies have been conducted in two countries (Mexico and Costa Rica) and in two vegetation types (RF 41% and 33%). It is therefore essential that studies are carried out in other countries and other vegetation types where Baird’s tapirs are found. This will help us to understand whether these animals make efficient use of the resources available to them in each season. Furthermore, it should be noted that some of the studies in Mexico and Costa Rica were conducted many years ago, and as a result, would need to be repeated, as many of these sites may have been altered by climate change or changes in land use.
In order to analyse the influence of seasonality on diet, it is best to consider the type of technique used separately. Studies such as those by Naranjo [43], Naranjo and Cruz-Aldán [48], and Reyes-Alcaraz [53] demonstrate significant discrepancies in values obtained for the same dietary component when the two techniques are employed.
Fibre may be present in greater quantities or more frequently in Baird’s tapir diet during the dry season because the quality of forage is lowest at this time of year [83]. This is because plants invest more in structural carbohydrates during the dry season, resulting in a higher carbon: nitrogen ratio [84]. However, the production of fruits of many tropical trees coincides with the dry season [85], meaning that the consumption of some fruits, which are rich in dry matter [80], could also increase.
All studies that used the frequency per occurrence technique showed that the percentage of leaves is higher during the rainy season, as did two-thirds of the studies that used the weighing technique. Only in two studies was the percentage of leaves higher in the dry season [43,45]. Interestingly, in Naranjo’s [43] study in Costa Rica, the results differ according to the technique used, as higher values are reported with the weighing technique than with the frequency per occurrence technique.
Lower leaf consumption during the dry season could be related to deciduousness, which occurs in many tropical forest trees [86]. This phenomenon is an adaptation to water stress, which induces the fall of leaves and limits the growth of new shoots and leaves [86]. It is therefore expected that Baird’s tapirs living in drier areas will consume fewer leaves compared to tapirs living in more humid areas, or that the species consumed in a given area will differ more or less between seasons according to their deciduousness. Moreover, certain species may possess more fibrous leaves during the dry season [87], which would consequently influence the research results.
Quantifying fruits is the most challenging aspect of the process, regardless of the method used. Most studies report a higher percentage of fruit in the diet during the dry season, with both the frequency per occurrence and the weighing methods. Restrepo and Betancourt [39] highlight that this increase in the percentage of fruit may be attributable to the samples being collected during the dry season, when fruit is more abundant. This increased fruit consumption during the dry season has also been documented in the lowland tapir in the Peruvian Amazon [88] and in French Guiana [77]. However, there are also contradictory results, such as those of Naranjo [43] and Foerster and Vaughan [30], both conducted in the same study area (Corcovado National Park in Costa Rica). Naranjo [43] obtained higher values for fruit in the dry season by analysing faeces, while Foerster and Vaughan [35] obtained higher values in the rainy season through direct observation. This could be caused by the underestimation of the amount of fruit consumed in the former study, as some fruits (especially those with high water content) are almost completely digested and may be undetectable in faeces.
5. Conclusions
Only a few studies have been conducted on the diet of the Baird’s tapir in the last 10 years, even though there are still many regions of Mesoamerica where virtually nothing is known about these topics. Moreover, information on the sites where studies have been conducted in the past should be updated, as many of these sites may have been altered due to human activity or climate change. The results of studies analysing faeces should be treated with caution, as these quantify the least digestible components rather than all the components in the diet. Studies on diet should be conducted over much longer periods to account for fluctuating plant phenology caused by natural climate cycles (e.g., El Niño). Such long study periods require cheap, automated techniques, such as camera trap monitoring for plant phenology. In addition to molecular techniques (DNA metabarcoding) and stable isotopes, which facilitate the analysis of Baird’s tapirs’ diets from a different perspective. We believe that such studies are necessary to understand how tapirs utilise available resources, respond to environmental changes, move in their habitat, and affect forest dynamics.
Supplementary Materials
The following supporting information can be downloaded at https://www.mdpi.com/article/10.3390/wild3020015/s1, Table S1. Studies with reports on plants consumed by Baird’s tapir in its geographic range; Table S2. List of plants consumed by Baird’s tapirs (Tapirus bairdii) in its geographic range, study sites, and references. Based on 25 studies published between 1978 and 2024. BZ = Belize, COL = Colombia, CR = Costa Rica, GT = Guatemala, HND = Honduras, MX = Mexico, NI = Nicaragua, and PAN = Panama.
Author Contributions
Conceptualization, J.P.-F.; methodology, J.P.-F., S.C. and D.G.-S.; formal analysis, J.P.-F.; investigation, J.P.-F.; data curation, J.P.-F.; writing—original draft preparation, J.P.-F., S.C. and D.G.-S.; writing—review and editing, J.P.-F., S.C. and D.G.-S.; supervision, J.P.-F. All authors have read and agreed to the published version of the manuscript.
Funding
This research received no external funding.
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
The data supporting this study are available within the article and its cited references.
Acknowledgments
The map in Figure 1 was produced by Holger Weissenberger. We are very grateful with Nereyda Estrada and Manolo García for sharing materials. J.P.-F. was supported by a doctoral scholarship (361517) granted by the Mexican government through the Secretaría de Ciencia, Humanidades, Tecnología e Innovación (SECIHTI).
Conflicts of Interest
The authors declare no conflicts of interest.
References
- Koerner, S.E.; Smith, M.D.; Burkepile, D.E.; Hanan, N.P.; Avolio, M.L.; Collins, S.L.; Knapp, A.K.; Lemoine, N.P.; Forrestel, E.J.; Eby, S.; et al. Change in dominance determines herbivore effects on plant biodiversity. Nat. Ecol. Evol. 2018, 2, 1925–1932. [Google Scholar] [CrossRef] [Scilit]
- Hibert, F.; Taberlet, P.; Chave, J.; Scotti-Saintagne, C.; Sabatier, D.; Richard-Hansen, C. Unveiling the diet of elusive rainforest herbivores in next generation sequencing era? The tapir as a case study. PLoS ONE 2013, 8, e60799. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ripple, W.J.; Chapron, G.; López-Bao, J.V.; Durant, S.M.; Macdonald, D.W.; Lindsey, P.A.; Bennett, E.L.; Beschta, R.L.; Bruskotter, J.T.; Campos-Arceiz, A.; et al. Saving the world’s terrestrial megafauna. BioScience 2016, 66, 807–812. [Google Scholar] [CrossRef] [Scilit]
- Vallentine, J.F. Grazing Management; Academic Press: San Diego, CA, USA, 1990. [Google Scholar]
- Harrison, K.A.; Bardgett, R.D. Impacts of grazing and browsing by large herbivores on soil and soil biological properties. In The Ecology of Browsing and Grazing; Ecological Studies; Gordon, I.J., Prins, H.H.T., Eds.; Springer: Berlin, Germany, 2008; Volume 195, pp. 201–216. [Google Scholar]
- De Vos, A. Ecological conditions affecting the production of wild herbivorous mammals on grasslands. In Advance in Ecological Research; Cragg, J.B., Ed.; Academic Press: London, UK, 1969; Volume 6, pp. 137–183. [Google Scholar]
- McNaughton, S.J.; Georgiadis, N.J. Ecology of African grazing and browsing mammals. Annu. Rev. Ecol. Syst. 1986, 16, 39–66. [Google Scholar] [CrossRef]
- Langer, P. The Mammalian Herbivore Stomach: Comparative Anatomy, Function and Evolution; Gustav Fischer Verlag: New York, NY, USA, 1988. [Google Scholar]
- Belovsky, G.E. Optimal foraging and community structure: The allometry of herbivore food selection and competition. Evol. Ecol. 1997, 11, 641–672. [Google Scholar] [CrossRef] [Scilit]
- Kelly, J.F. Stable isotopes of carbon and nitrogen in the study of avian and mammalian trophic ecology. Can. J. Zool. 2000, 78, 1–27. [Google Scholar] [CrossRef]
- Litvaitis, J.A. Investigating food habits of terrestrial vertebrates. In Research Techniques in Animal Ecology: Controversies and Consequences; Boitani, L., Fullere, T.K., Eds.; Columbia University Press: New York, NY, USA, 2000; pp. 165–190. [Google Scholar]
- MacFadden, B.J. Cenozoic mammalian herbivores from the Americas: Reconstructing ancient diets and terrestrial communities. Annu. Rev. Ecol. Evol. Syst. 2000, 31, 33–59. [Google Scholar] [CrossRef] [Scilit]
- Villar, N.; Medici, E.P. Large wild herbivores slow down the rapid decline of plant diversity in a tropical forest biodiversity hotspot. J. App. Ecol. 2021, 58, 2361–2370. [Google Scholar] [CrossRef] [Scilit]
- Venter, J.A.; Kalule-Sabiti, M.J. Diet composition of the large herbivores in Mkambati Nature Reserve, Eastern Cape, South Africa. S. Afr. J. Wildl. Res. 2016, 46, 49–56. [Google Scholar] [CrossRef] [Scilit]
- Ritchie, M.E. Optimal foraging and fitness in Columbian ground squirrels. Oecologia 1990, 82, 56–67. [Google Scholar] [CrossRef] [Scilit]
- White, R.G. Foraging patterns and their multiplier effects on productivity of northern ungulates. Oikos 1983, 40, 377–384. [Google Scholar] [CrossRef] [Scilit]
- Ripple, W.J.; Newsome, T.M.; Wolf, C.; Dirzo, R.; Everatt, K.T.; Galetti, M.; Hayward, M.W.; Kerley, G.I.H.; Levi, T.; Lindsey, P.A.; et al. Collapse of the world’s largest herbivores. Sci. Adv. 2015, 1, e1400103. [Google Scholar] [CrossRef] [Scilit]
- Goldberg, R.A.; Conway, C.J.; Tank, D.C.; Andrews, K.R.; Gour, D.S.; Waits, L.P. Diet of a rare herbivore based on DNA metabarcoding of feces: Selection, seasonality, and survival. Ecol. Evol. 2020, 10, 7627–7643. [Google Scholar] [CrossRef] [Scilit]
- O’Farrill, G.; Galetti, M.; Campos-Arceiz, A. Frugivory and seed dispersal by tapirs: An insight on their ecological role. Integr. Zool. 2013, 8, 4–17. [Google Scholar] [CrossRef] [Scilit]
- Paolucci, L.N.; Pereira, R.L.; Rattis, L.; Silvério, D.V.; Marques, N.C.S.; Macedo, M.N.; Brando, P.M. Lowland tapirs facilitate seed dispersal in degraded Amazonian forests. Biotropica 2019, 51, 245–252. [Google Scholar] [CrossRef] [Scilit]
- Nowak, R.M. Walker’s Mammals of the World, 6th ed.; Johns Hopkins University Press: Baltimore, MD, USA, 1999. [Google Scholar]
- Fragoso, J.M.V.; Huffman, J. Seed-dispersal and seedling recruitment patterns by the last Neotropical megafaunal element in Amazonia, the tapir. J. Trop. Ecol. 2000, 16, 369–385. [Google Scholar] [CrossRef] [Scilit]
- Cordeiro, J.L.P.; Fragoso, J.M.V.; Crawshaw, D.; Oliveira, L.F.B. Lowland tapir distribution and habitat loss in South America. PeerJ 2016, 4, e2456. [Google Scholar] [CrossRef] [Scilit]
- Yanez-Montalvo, A.; Gaona, O.; de León-Lorenzana, A.; Águila, B.; Falcón, L.; Neri-Barrios, C.X.; Pérez-Flores, J. What can tapir poop teach us about healthy forests? Front. Young Minds 2023, 11, 947799. [Google Scholar] [CrossRef] [Scilit]
- García, M.; Jordan, C.; O’Farrill, G.; Meyer, N.; Estrada, N.; Leonardo, R.; Naranjo, E.; Simons, Á.; Herrera, A.; Urgilés, C.; et al. Tapirus bairdii. IUCN Red List. Threat. Species 2016, eT214471A45173340. [Google Scholar] [CrossRef] [Scilit]
- Myers, N.; Mittermeier, R.A.; Mittermeier, C.G.; da Fonseca, G.A.; Kent, J. Biodiversity hotspots for conservation priorities. Nature 2000, 403, 853–858. [Google Scholar] [CrossRef] [Scilit]
- de Albuquerque, F.S.; Benito, B.; Beier, P.; Assunção-Albuquerque, M.J.; Cayuela, L. Supporting underrepresented forests in Mesoamerica. Nat. Conserv. 2015, 13, 152–158. [Google Scholar] [CrossRef] [Scilit]
- Reyna-Hurtado, R.; Sanvicente-López, M.; Pérez-Flores, J.; Carrillo-Reyna, N.; Calmé, S. Insights into the multiannual home range of a Baird’s tapir (Tapirus bairdii) in the Maya Forest. Therya 2016, 7, 271–276. [Google Scholar] [CrossRef] [Scilit]
- Yanez-Montalvo, A.; Gaona, O.; Águila, B.; Arias-Domínguez, N.; Falcón, L.I.; Pérez-Flores, J. Tapirus bairdii-associated fecal microbiome from a critical conservation area: Calakmul, México. Curr. Microbiol. 2021, 78, 2648–2659. [Google Scholar] [CrossRef] [Scilit]
- Foerster, C.R.; Vaughan, C. Home range, habitat use, and activity of Baird’s tapir in Costa Rica. Biotropica 2002, 34, 423–437. [Google Scholar] [CrossRef] [Scilit]
- Pérez-Flores, J.; Weissenberger, H.; López-Cen, A.; Calmé, S. Environmental factors influencing the occurrence of unhealthy tapirs in the southern Yucatan Peninsula. EcoHealth 2020, 17, 359–369. [Google Scholar] [CrossRef] [Scilit]
- Tobler, M.W. Habitat use and diet of Baird’s Tapirs (Tapirus bairdii) in a Montane Cloud Forest of the Cordillera de Talamanca, Costa Rica. Biotropica 2002, 34, 468–474. [Google Scholar] [CrossRef] [Scilit]
- Tobler, M.W.; Naranjo, E.; Lira-Torres, I. Habitat preferences, feeding habits and conservation of Baird’s tapir in Neotropical montane oak forests. In Ecology and Conservation of Neotropical Montane Oak Forests; Kappelle, M., Ed.; Springer: Berlin, Germany, 2006; pp. 347–361. [Google Scholar]
- Foerster, C.R. Ecología de la Danta Centroamericana Tapirus bairdii en un Bosque Húmedo Tropical de Costa Rica. Master’s Thesis, Universidad Nacional, Heredia, Costa Rica, 1998. [Google Scholar]
- Foerster, C.R.; Vaughan, C. Diet and foraging behavior of a female Baird’s tapir (Tapirus bairdii) in a Costa Rican lowland rainforest. Cuad. Inv. UNED 2015, 7, 259–267. [Google Scholar]
- Sourial, N.; Wolfson, C.; Zhu, B.; Quail, J.; Fletcher, J.; Karunananthan, S.; Bandeen-Roche, K.; Béland, F.; Bergman, H. Correspondence analysis is a useful tool to uncover the relationships among categorical variables. J. Clin. Epidemiol. 2010, 63, 638–646. [Google Scholar] [CrossRef] [Scilit]
- R Core Team. R: A Language and Environment for Statistical Computing, Version 4.5.2.; [Computer software]; R Foundation for Statistical Computing: Vienna, Austria, 2025; Available online: https://www.R-project.org/ (accessed on 15 January 2026).
- Fragoso, J.M.V. The Habitat Preferences and Social Structure of Tapirs. Master’s Thesis, University of Toronto, Toronto, ON, Canada, 1987. [Google Scholar]
- Restrepo, H.F.; Betancourt, O. Confirmación de la presencia del tapir centroamericano (Tapirus bairdii) en Colombia, y studio preliminar sobre algunos aspectos de su historia natural en el Parque Nacional Natural Los Katíos. Tapir Conserv. Newsl. IUCN/SSC Tapir Spec. Group 2006, 15, 29–36. [Google Scholar]
- Mejía-Correa, S.; Díaz-Martínez, A.; Molina, R. Densidad y hábitos alimentarios de la danta Tapirus bairdii en el Parque Nacional Natural Los Katios, Colombia. Tapir Conserv. Newsl. IUCN/SSC Tapir Spec. Group 2014, 23, 16–23. [Google Scholar]
- Janzen, D.H. Wild plant acceptability to a captive Costa Rican Baird’s tapir. Brenesia 1982, 19/20, 99–128. [Google Scholar]
- Williams, K.D. The Central American Tapir (Tapirus bairdii Gill) in Northwestern Costa Rica. Doctoral Dissertation, Michigan State University, East Lansing, MI, USA, 1984. [Google Scholar]
- Naranjo, E. Hábitos de alimentación del tapir (Tapirus bairdii) en un bosque tropical húmedo de Costa Rica. Vida Silv. Neotrop. 1995, 4, 32–37. [Google Scholar]
- Carvajal, J.P.; Marín-Pacheco, P.; Espinoza-Chacón, A.; Rohrmoser-Steinvorth, F.; Pérez-Pérez, C. Nuevos registros de plantas comidas por el tapir, Tapirus bairdii (Perissodactyla: Tapiridae), en el Parque Nacional Braulio Carrillo, Costa Rica. Cuad. Inv. UNED 2020, 12, e2771. [Google Scholar] [CrossRef] [Scilit]
- García, J.M. Caracterización de la Dieta y Habitat del Tapir (Tapirus bairdii Gill, 1865) en Ecosistemas Ribereños del Parque Nacional Laguna Lachuá, Cobán, AltaVerapaz, Guatemala. Bachelor’s Thesis, Universidad de San Carlos Guatemala, Guatemala City, Guatemala, 2006. [Google Scholar]
- Estrada, N. Estudio del Danto (Tapirus bairdii) en el Parque Nacional Sierra de Agalta, Olancho, Honduras; International Resources Group: Washington, DC, USA, 2006. [Google Scholar]
- Dirzo, R.; Miranda, A. Altered Patterns of Herbivory and Diversity in the Forest Understory: A Case Study of the Possible Consequences of Contemporary Defaunation; Price, P.W., Lewinsohn, T.M., Wilson, G., Benson, W.W., Eds.; Wiley and Sons: New York, NY, USA, 1991; pp. 273–287. [Google Scholar]
- Naranjo, E.; Cruz-Aldán, E. Ecología del tapir (Tapirus bairdii) en la Reserva de la Biosfera La Sepultura, Chiapas, México. Acta Zool. Mex. 1998, 73, 111–125. [Google Scholar] [CrossRef] [Scilit]
- Cruz-Aldán, E. Hábitos Alimentarios e Impacto de la Actividad Humana Sobre el Tapir en la Reserva de la Biosfera La Sepultura, Chiapas, México. Master’s Thesis, El Colegio de la Frontera Sur, San Cristobal de las Casas, Mexico, 2001. [Google Scholar]
- Lira-Torres, I.; Naranjo, E.; Güiris-Andrade, M.; Cruz-Aldán, E. Ecología de Tapirus bairdii (Perissodactyla: Tapiridae) en la Reserva de la Biosfera El Triunfo (Polígono I), Chiapas, México. Acta Zool. Mex. 2004, 20, 1–21. [Google Scholar] [CrossRef] [Scilit]
- Jiménez, D. Reporte de Investigación del Tapir Centroamericano (Tapirus bairdii) Como Dispersor de Semillas. Bachelor’s Thesis, El Colegio de la Frontera Sur, San Cristóbal de las Casas, Mexico, 2006. [Google Scholar]
- Rivadeneyra, E. Hábitos Alimentarios del Tapir (Tapirus bairdii) en el Sector sur de la Reserva de la Biosfera Montes Azules. Bachelor’s Thesis, Universidad Autónoma de Yucatán, Mérida, Mexico, 2007. [Google Scholar]
- Reyes-Alcaraz, L. Descripción de Habitat y Dieta del Tapir Centroamericano Tapirus bairdii Gill, 1865, en el Ejido La Fortaleza, Municipio Santa María Chimalapa, Oaxaca, México. Bachelor’s Thesis, Universidad Nacional Autónoma de México, Mexico City, Mexico, 2008. [Google Scholar]
- Pérez-Cortez, S.; Matus-Pérez, E.S. El tapir Tapirus bairdii en la región sureste del Área de Protección de Flora y Fauna Bala’an Ka’ax, Quintana Roo, México. Therya 2010, 1, 137–144. [Google Scholar] [CrossRef] [Scilit]
- Camargo-Sanabria, A.A.; Mendoza, E. Interactions between terrestrial mammals and the fruits of two neotropical rainforest tree species. Acta Oecologica 2016, 73, 45–52. [Google Scholar] [CrossRef] [Scilit]
- Granados-Pérez, A. Presencia de Tapir (Tapirus bairdii) en el Ejido La Lucha Dos, Othón Pompeyo Balnco, Quintana Roo. Bachelor’s Thesis, Universidad Autónoma Agraria Antonio Narro, Coahuila, Mexico, 2017. [Google Scholar]
- Pérez-Flores, J. Estudios Relacionados con la Salud del Tapir Centroamericano (Tapirus bairdii) en el Sureste de México. Doctoral Dissertation, El Colegio de la Frontera Sur, Chetumal, Mexico, 2020. [Google Scholar]
- Puc-Sánchez, J.I.; Camargo-Sanabria, A.A.; Mendoza, E. Predation of oak acorns by Baird’s tapir one of the last remnants of mountain cloud forest in Southern Mexico. Food Webs 2023, 37, e00312. [Google Scholar] [CrossRef] [Scilit]
- Domeiz-Dambus, J.A.; Smith-Chow, H.H.; Cordón-Suárez, E. Hábitat potencial del Danto (Tapirus bairdii) en la Costa caribe Norte de Nicaragua. Rev. Univ. Caribe 2017, 18, 66–73. [Google Scholar] [CrossRef] [Scilit]
- Terwilliger, V.T. Natural history of Baird’s tapir on Barro Colorado Island, Panama Canal Zone. Biotropica 1978, 10, 211–220. [Google Scholar] [CrossRef] [Scilit]
- Capece, P.I.; Aliaga-Rossel, E.; Jansen, P.A. Viability of small seeds found in feces of the Central American tapir on Barro Colorado Island, Panama. Int. Zool. 2013, 8, 57–62. [Google Scholar] [CrossRef] [Scilit]
- DeSantis, L.G. Stable istope ecology of extant tapirs from the Americas. Biotropica 2011, 43, 746–754. [Google Scholar] [CrossRef] [Scilit]
- Hibert, F.; Sabatier, D.; Andrivot, J.; Scotti-Saintagne, C.; Gonzalez, S.; Prévost, M.-F.; Grenand, P.; Chave, J.; Caron, H.; Richard-Hansen, C. Botany, genetics and ethnobotany: A crossed investigation on the elusive tapir’s diet in French Guiana. PLoS ONE 2011, 6, E25850. [Google Scholar] [CrossRef] [Scilit]
- Prado, H.M. Feeding ecology of five Neotropical ungulates: A critical review. Oecologia Aust. 2013, 17, 459–473. [Google Scholar] [CrossRef] [Scilit]
- van der Reis, A.L.; Norrie, C.R.; Jeffs, A.G.; Lavery, S.D.; Carroll, E.L. Genetic and particle modelling approaches to assessing population connectivity in a deep sea lobster. Sci. Rep. 2022, 12, 16783. [Google Scholar] [CrossRef] [Scilit]
- Cruz-Cano, R.; Kolb, M.; Saldaña-Vázquez, R.A.; Bretón-Deval, L.; Cruz-Cano, N.; Aldama-Cervantes, A. Existing evidence on the use of environmental DNA as an operational method for studying rivers: A systematic map and thematic synthesis. Environ. Evid. 2024, 13, 2. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Abwe, E.E.; Morgan, B.J.; Doudja, R.; Kentatchime, F.; Mba, F.; Dadjo, A.; Venditti, D.M.; Mitchell, M.W.; Fosso, B.; Mounga, A.; et al. Dietary ecology of the Nigeria-Cameroon chimpanzee (Pan troglodytes ellioti). Int. Primatol. 2020, 41, 81–104. [Google Scholar] [CrossRef] [Scilit]
- Yamagiwa, J.; Basabose, A.K. Diet and seasonal changes in sympatric gorillas and chimpanzees at Kahuzi–Biega National Park. Primates 2006, 47, 74–90. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- McLennan, M.R. Diet and feeding ecology of chimpanzees (Pan troglodytes) in Bulindi, Uganda: Foraging Strategies at the Forest–Farm Interface. Int. J. Primatol. 2013, 34, 585–614. [Google Scholar] [CrossRef] [Scilit]
- Garnick, S.; Barboza, P.S.; Walker, J.W. Assessment of animal-based methods used for estimating and monitoring rangeland herbivore diet composition. Rangel. Ecol. Manag. 2018, 71, 449–457. [Google Scholar] [CrossRef] [Scilit]
- Wallmo, O.C.; Neff, D.J. Direct observations of tamed deer to measure their consumption of natural forage. In Range and Wildlife Habitat Evaluation—A Research Symposium; US Department of Agriculture and Forest Service Miscellaneous Publication no. 1147: Washington, DC, USA, 1970. [Google Scholar]
- Mosquera-Guerra, F.; Moreno-Niño, N.; Barreto, S.; Pascual, D.A. Habitat suitability and representation of the potential distribution of the lowland tapir (Tapirus terrestris) within land cover types and protected areas of eastern Colombia. Mamm. Res. 2024, 69, 507–518. [Google Scholar] [CrossRef] [Scilit]
- Simpson, B.K.; Shukor, M.N.; Magintan, D. Food selection of the Malayan tapir (Tapirus indicus) under semi-wild conditions. AIP Conf. Proc. 2013, 1571, 317–324. [Google Scholar] [CrossRef] [Scilit]
- Beech, E.; Alvarez-Clare, S.; Brewer, S.; Coronado, I.; Ledis-Linares, J.; MacVean, A.L.; Martínez-Salas, E.; Machuca-Machuca, K.; Redonda-Martínez, R.; Rodríguez-Delcid, D.; et al. Comprehensive tree assessments for prioritizing conservation action in Mesoamerica. Plants People Planet 2025, 7, 1813–1823. [Google Scholar] [CrossRef] [Scilit]
- Matola, S.; Cuaron, A.D.; Rubio-Togler, H. Status and action plan of Baird’s tapir. In Tapirs: Status Survey and Conservation Action Plan; Brooks, D.M., Bodmer, R.E., Matola, S., Eds.; IUCN/SSC Tapir Specialist Group: Cambridge, UK, 1997; pp. 29–45. [Google Scholar]
- Naranjo, E.; Vaughan, C. Ampliación del ámbito altitudinal del tapir centroamericano (Tapirus bairdii). Rev. Biol. Trop. 2000, 48, 724. [Google Scholar]
- Henry, O.; Feer, F.; Sabatier, D. Diet of the lowland tapir (Tapirus terrestris L.) in French Guiana. Biotropica 2000, 32, 364–368. [Google Scholar] [CrossRef] [Scilit]
- Shanahan, M.; So, S.; Gompton, S.G.; Gorlett, R. Fig-eating by vertebrate frugivores: A global review. Biol. Rev. 2001, 76, 529–572. [Google Scholar] [CrossRef] [Scilit]
- Ruenes-Morales, M.R.; Montañez, E.P.I.; Ferrer, M.M.; Jiménez, O.J.J.; González, I.R.E.; González, I.A.J.A. Spondias mombin L. Spondias purpurea L. Spondias radlkoferi J.D. Smith Anacardiaceae. In Ethnobotany of the Mountain Regions of Mexico; Ethnobotany of Mountain Regions; Casas, A., Blancas, V.J.J., Eds.; Springer Cham: Nueva York, NY, USA, 2022; pp. 1–17. [Google Scholar]
- Clauss, M.; Lang-Deuerling, S.B.; Baumgartner, K.; Medici, E.P.; Janssens, G.P.J.; Kienzle, E.; Hummel, J. Nutrient digestibility in zoo-kept tapirs (Tapirus spp.) as compared to other herbivores. J. Anim. Physiol. Anim. Nutr. 2024, 109, 867–880. [Google Scholar] [CrossRef] [Scilit]
- Pinto, L.P.; Pires, M.M.; Cademartori, C.V.; Périco, E. Endozoochory by lowland tapirs improves seed germinability and accelerates germination time of native plants in an Amazon-Cerrado transition restoration area. Acta Amaz. 2025, 55, e55bc24316. [Google Scholar] [CrossRef] [Scilit]
- Bello, C.; Galetti, M.; Pizo, M.A.; Magnano, L.F.S.; Rocha, M.F.; Lima, R.A.F.; Peres, C.A.; Ovaskainen, O.; Jordano, P. Defaunation affects carbon storage in tropical forests. Sci. Adv. 2015, 1, e1501105. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hernández-Hernández, M.; López-Ortiz, S.; Jarillo-Rodríguez, J.; Ortega-Jiménez, E.; Pérez-Elizalde, S.; Díaz-Rivera, P.; Crosby-Galván, M.M. Forage yield and nutritional quality in Leucaena leucocephala and Megathyrsus maximus cv. Tanzania in an intensive silvopastoral system. Rev. Mex. Cienc. Pec. 2020, 11, 53–69. [Google Scholar] [CrossRef] [Scilit]
- Ahrestani, F.S.; Heitkönig, I.M.A.; Prins, H.H.T. Diet and habitat-niche relationships within an assemblage of large herbivores in a seasonal tropical forest. J. Trop. Ecol. 2012, 28, 385–394. [Google Scholar] [CrossRef] [Scilit]
- Luna-Nieves, A.L.; Meave, J.A.; Cerdeira-Morellato, L.P.; Ibarra-Manríquez, G. Reproductive phenology of useful seasonally dry tropical forest trees: Guiding patterns for seed collection and plant propagation in nurseries. For. Ecol. Manag. 2017, 393, 52–62. [Google Scholar] [CrossRef] [Scilit]
- Singh, K.P.; Kushwaha, C.P. Deciduousness in tropical trees and its potential as indicator of climate change: A review. Ecol. Indic. 2016, 69, 699–706. [Google Scholar] [CrossRef] [Scilit]
- Wang, Y.; Yang, D.; Vargas, G.; Hao, G.; Powers, J.S.; Ke, Y.; Wang, Q.; Zhang, Y.; Zhang, J. Leaf habitat differentiation explains trait tradeoffs across savanna woody plants. For. Ecosyst. 2024, 11, 100190. [Google Scholar] [CrossRef] [Scilit]
- Bodmer, R.E. Fruit patch size and frugivory in the lowland tapir (Tapirus terrestris). J. Zool. 1990, 222, 121–128. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.