


Abstract
Cirsium vulgare (Asteraceae) is a newly emerged invasive species in Yunnan Province, China, and its phytotoxic potential has not yet been studied. This study was conducted to explore potential allelopathic effects of C. vulgare and to identify its flavonoid and phenolic acid compounds. Four aqueous extracts (roots, stems, leaves, and flower/fruit heads) of C. vulgare exhibited high inhibitory activity against the germination and seedling growth of Bidens pilosa and Digitaria sanguinalis. The inhibition rates of germination rate, germination index, root length, shoot length, and biomass of both species increased significantly with increasing concentrations, with B. pilosa being more inhibited than D. sanguinalis. Extracts from leaves and flower/fruit heads yielded the strongest inhibition, followed by stem extracts, with the lowest impact from root extracts. Flavonoids (65.41%) and phenolic acids (23.1%) collectively comprised 88.51% of all identified compounds. Thirty-eight flavonoid compounds and thirty phenolic acid compounds were selected for further analysis, representing 53.97% and 71.91% of the total content of flavonoids and phenolic acids, respectively. Many of the flavonoids and phenolic acids identified have been previously reported as known allelochemicals with possible allelopathic effects. This was the first study to show that the allelopathic potential of C. vulgare may aid its invasion and expansion.
1. Introduction
Invasive alien plant species are highly impactful and pose a major threat to global biodiversity loss [1]. They not only disrupt critical ecosystem services but also cause various negative impacts to socio-economic development [2,3,4]. Many invasive species dominate ecosystems owing to their rapid growth and strong physiological and ecological adaptability, and are frequently allelopathic [5,6,7,8]. A study of 524 invasive plant species found that over half (51.4%) the species produce allelochemicals, demonstrating the potential for allelopathy to significantly impact native species and crops worldwide [2]. Furthermore, allelopathy is commonly regarded as a main contributing factor in the success of these invasive exotics [6,9,10]. The novel weapon hypothesis [6] and allelopathic-driving hypothesis [8] demonstrate that invasive species may produce allelochemicals that can directly inhibit neighboring native plants or indirectly suppress native plants via disruption of beneficial below-ground microbial mutualisms, or altered soil resources. Therefore, studying the allelopathic potential of invasive plants is essential to understanding how they compete with crops and native species.
The biennial to short perennial herbaceous plant Cirsium vulgare (Savi) Ten. (Asteraceae) is native to Europe, western Asia, and North Africa [11,12]. Cirsium vulgare has expanded its range to cool-temperate, warm-temperate, and subtropical zones on every continent except Antarctica by thriving in human-altered habitats [13]. Consequently, it is regarded as one of the world’s most notorious invasive plants, being both highly impactful to the environment and geographically widespread [14,15,16]. This species thrives in various open and disturbed habitats, including arable field margins, roadsides, forest clearings, and pastures [12].
Cirsium vulgare was first recognized as a species of potential concern in Yunnan Province, southwestern China in 2022. A specimen was collected from Panlong District, Kunming City, and subsequently identified as C. vulgare through comprehensive literature review and expert opinion. It has been deposited in the Agricultural Environment and Resource Research Institute, Yunnan Academy of Agricultural Sciences, China. Further field investigations and monitoring across the province showed that C. vulgare is common in Kunming City, Yuxi City, Chuxiong City, and Qujing City, frequently invading farmland, wasteland, and managed public landscapes such as parks, roadsides, and green belts. iNaturalist records show that it also occurs in Guizhou Province. This species is characterized as an injurious weed due to its spiny stems and leaves that make it unpalatable to most stock, although seedlings or small rosettes may be eaten by sheep [12,14]. The robust taproot of C. vulgare allows its adaptability to diverse environmental conditions, particularly drought [12]. Cirsium vulgare can easily spread to surrounding areas by wind through numerous pappus hairs around seeds.
Cirsium species contain secondary metabolites such as flavonoids, phenolic acids, sterols, and aliphatic aldehydes [17,18,19,20], which are known to have various antioxidant and antibacterial activities [21,22,23]. Phenolic acids and flavonoids have been extensively studied for their allelopathic activity [24,25,26]. Phenolic allelochemicals mediate plant competition through the suppression of growth of other species, thereby influencing competitive interactions and thus affecting plant succession [27]. Previous studies have shown, using a range of extraction methods, that C. vulgare contains different phenolic acid and flavonoid compounds in various plant parts, and that these compounds have strong antioxidant activity [20,22,25]; however, no investigations into phytotoxic activity have been conducted.
This study hypothesized that C. vulgare may have strong competitiveness through its allelopathic potential. In order to explore the allelopathic mechanisms, the allelopathic potential of C. vulgare against two weed species, Bidens pilosa L. (Asteraceae) and Digitaria sanguinalis (L.) Scop. (Poaceae), which are widespread in China and commonly found in areas with C. vulgare, was investigated using aqueous extracts from the roots, stems, leaves, and flower/fruit heads of C. vulgare. Moreover, based on initial bioassay results and previous studies on phenolic acid and flavonoid compounds of C. vulgare [20,22,25], the overall phenolic acids and flavonoids from methanol extracts of C. vulgare leaves were explored by UPLC-MS analysis. Understanding the allelopathic mechanisms of the invasive plant C. vulgare is crucial for developing early detection and rapid response strategies for proactive management.
2. Results
2.1. Seed Germination and Seedling Growth
Seed germination and seedling growth of B. pilosa and D. sanguinalis varied significantly with plant part and concentration level of C. vulgare extracts, with a significant interaction effect (except for the germination index of B. pilosa) (p < 0.01) (Table 1 and Table 2). The germination rate and germination index of B. pilosa and D. sanguinalis were significantly inhibited by all four aqueous extracts of C. vulgare, with the highest inhibition rates by leaves and flower/fruit heads, followed by stems, and the lowest impact was seen from root extracts (Table 1). With increasing concentrations of the four aqueous extracts, inhibition was markedly increased, and the inhibitory rates of the germination index of the two test species were generally higher than those of germination rate. The inhibitory rates of germination rate and germination index of B. pilosa were generally higher than those of D. sanguinalis (Table 1).
Table 1.
Inhibitory rate (%) of Cirsium vulgare extracts on seed germination of Bidens pilosa and Digitaria sanguinalis.
Table 2.
Inhibitory rate (%) of Cirsium vulgare extracts on the growth of Bidens pilosa and Digitaria sanguinalis.
The four aqueous extracts of C. vulgare resulted in varying effects on the root length, shoot length, and biomass of B. pilosa and D. sanguinalis (Table 2). The four aqueous extracts of C. vulgare exhibited powerful inhibitory effects on seedling growth of the two test species (Table 2). The inhibitory rates of the aqueous extracts on the root length, shoot length, and biomass of B. pilosa and D. sanguinalis significantly increased with higher extract concentrations, with B. pilosa experiencing greater inhibition than D. sanguinalis. Against B. pilosa, extracts from leaves and flower/fruit heads of C. vulgare generally had the strongest inhibition effect, followed by stems, with the lowest inhibition from root extract. However, against D. sanguinalis, extracts from leaves generally had the strongest inhibition effect on the root length, shoot length, and biomass (Table 2).
2.2. Allelopathic Response Index
The measured allelopathic response index and the synthetical allelopathic index of the aqueous extracts of C. vulgare on seed germination and seedling growth of B. pilosa and D. sanguinalis varied, depending on plant parts, concentrations, and species (Table 3 and Table 4). All measured allelopathic response indices of the aqueous extracts of C. vulgare on B. pilosa and D. sanguinalis were significantly lower than 0 and were significantly reduced with increasing concentration. Comparing the allelopathic response index for the two bioassay species, germination rate was inhibited minimally more than germination index, with shoot and root length and biomass the highest inhibited, and the inhibitory rates of B. pilosa were generally higher than those of D. sanguinalis (Table 3 and Table 4). Comparing the synthetical allelopathic index values across both B. pilosa and D. sanguinalis, the magnitude of the inhibition was greatest for leaf and flower/fruit head extracts generally, with somewhat less inhibition for stem extracts, and the least inhibition by root extracts (Table 3 and Table 4).
Table 3.
Allelopathic response index of Bidens pilosa due to four aqueous extracts of Cirsium vulgare.
Table 4.
Allelopathic response index of Digitaria sanguinalis due to four aqueous extracts of Cirsium vulgare.
2.3. Identification of Flavonoid and Phenolic Acid Compounds
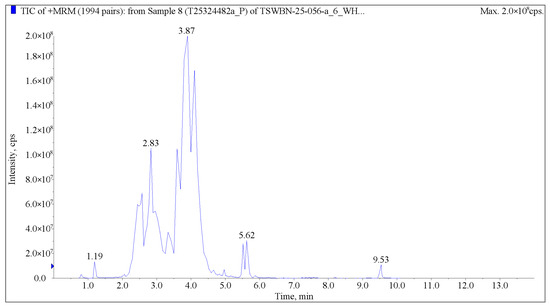
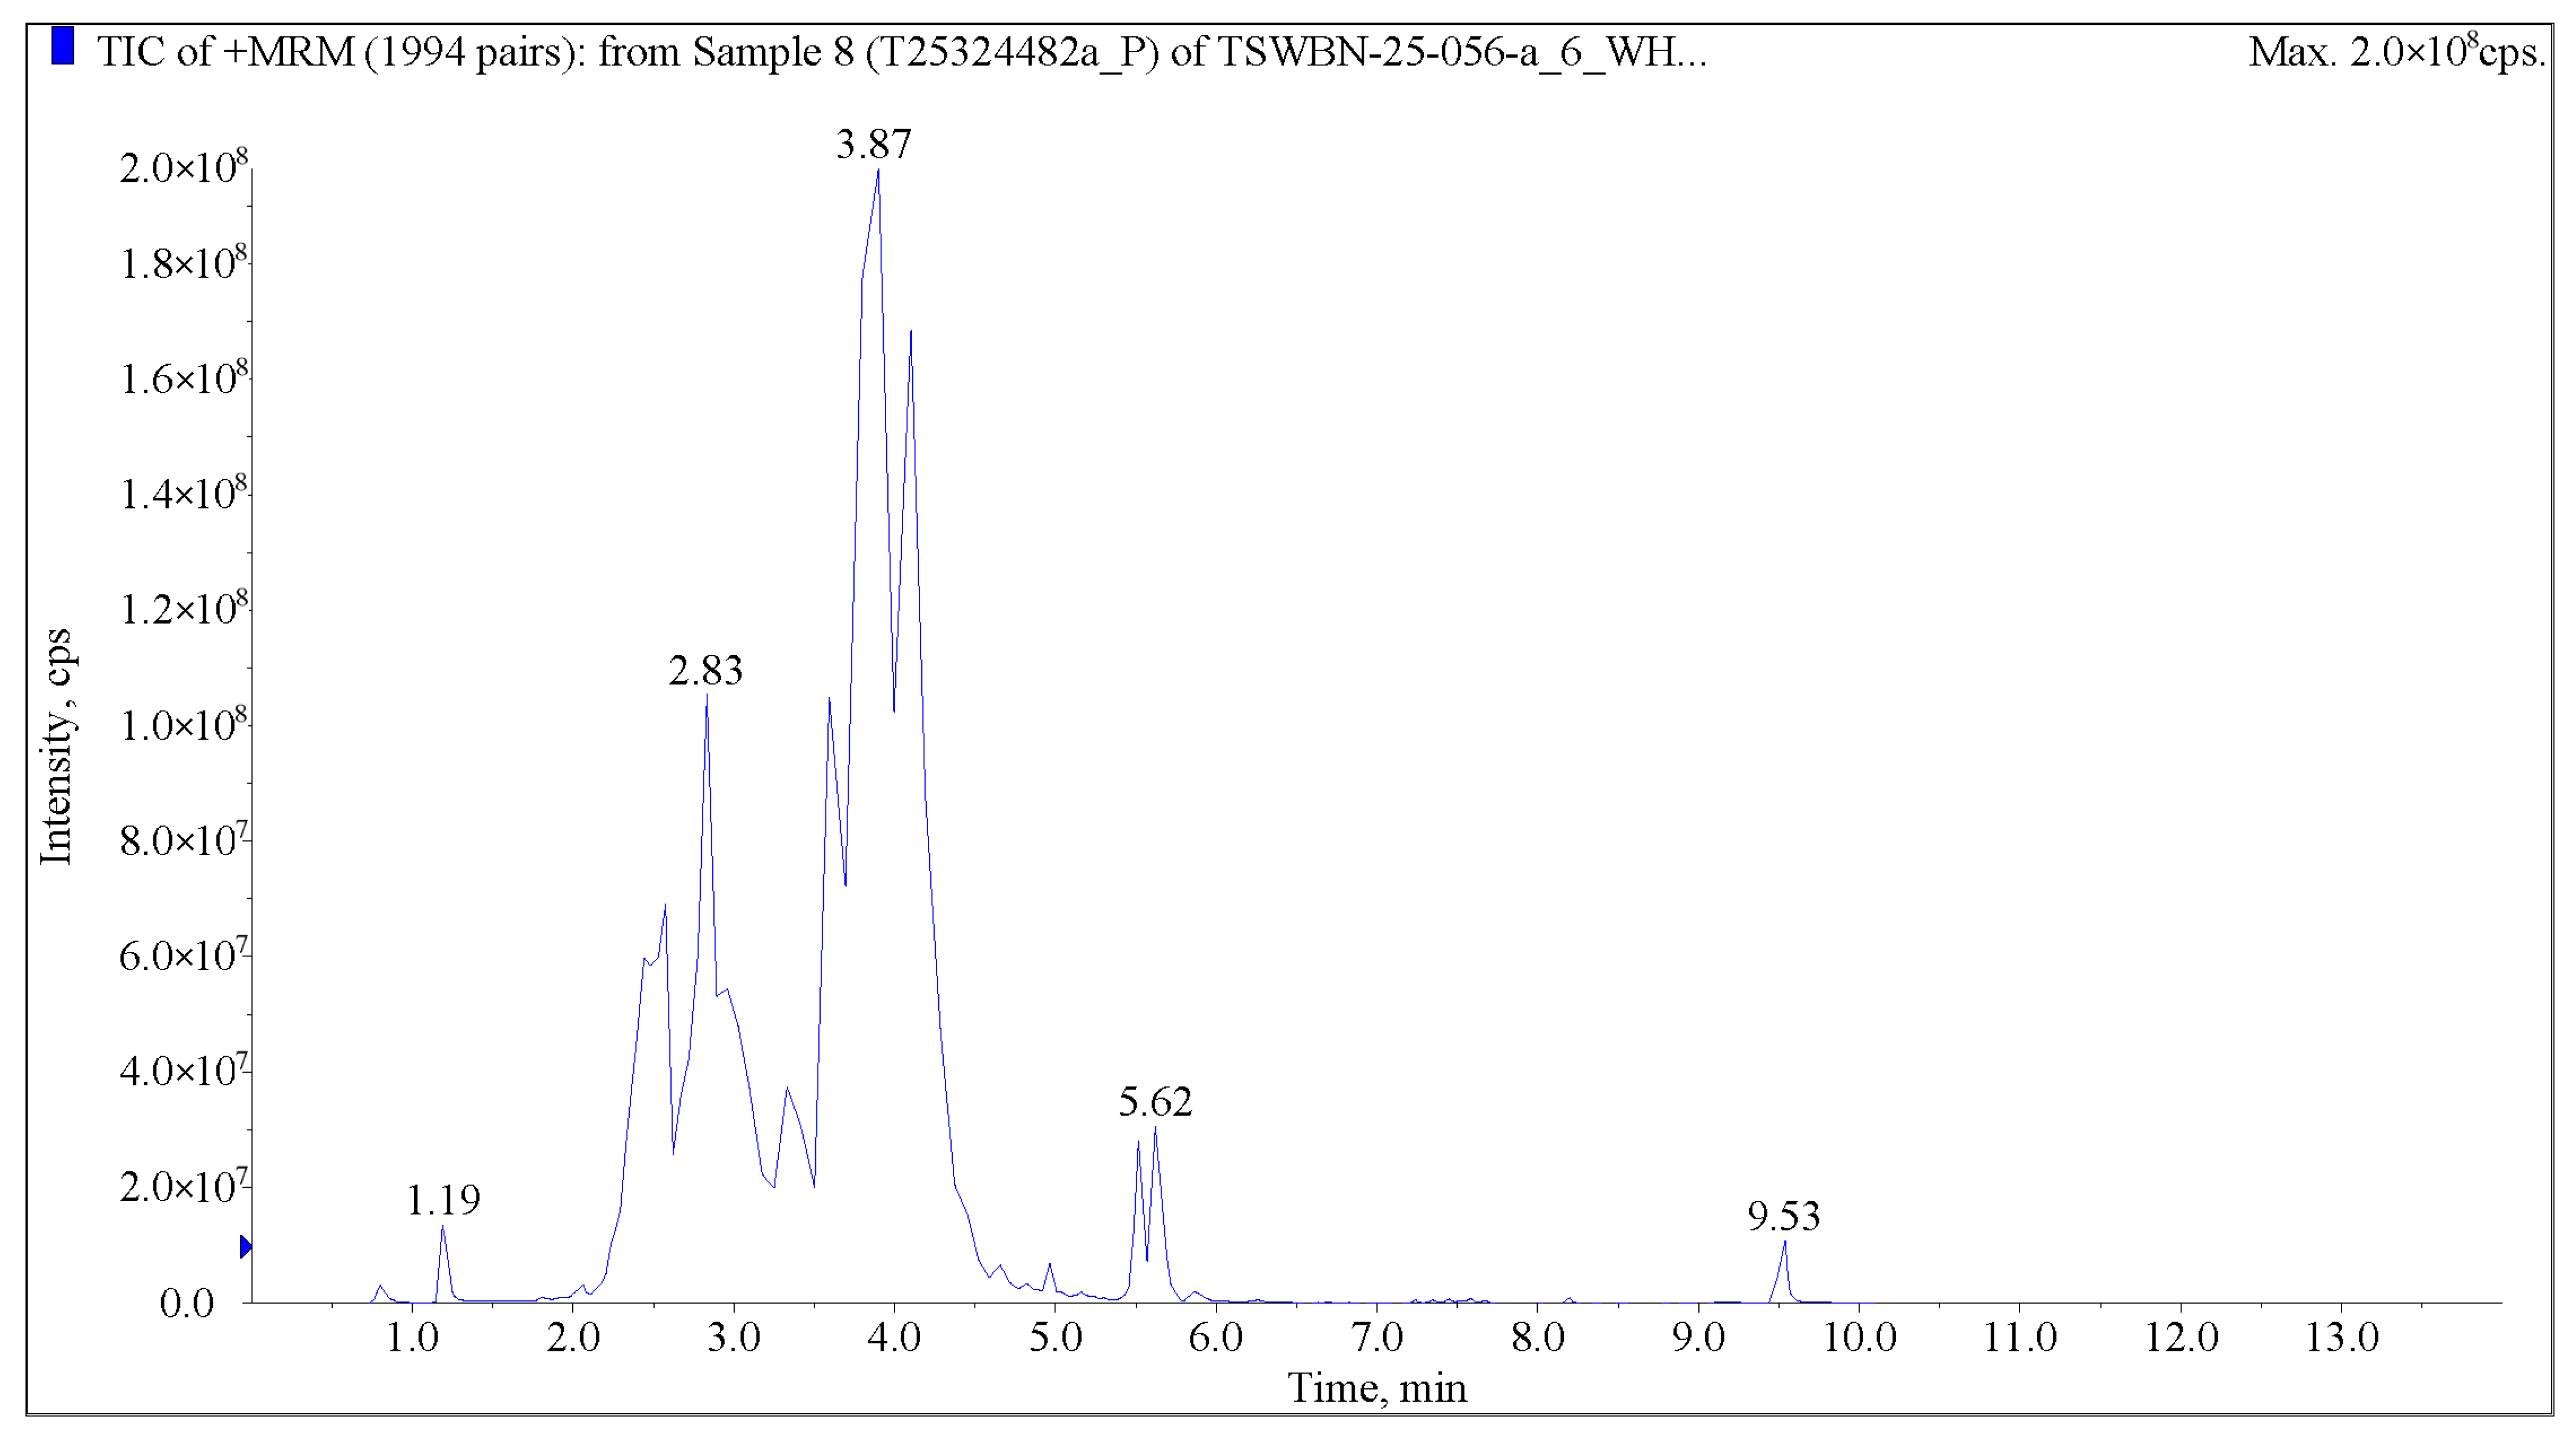
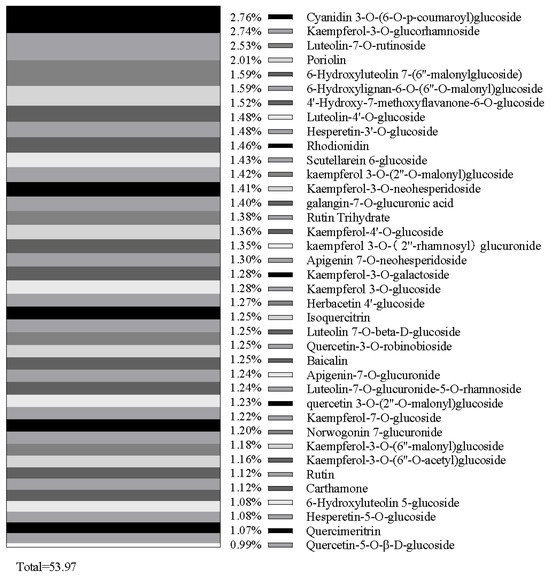
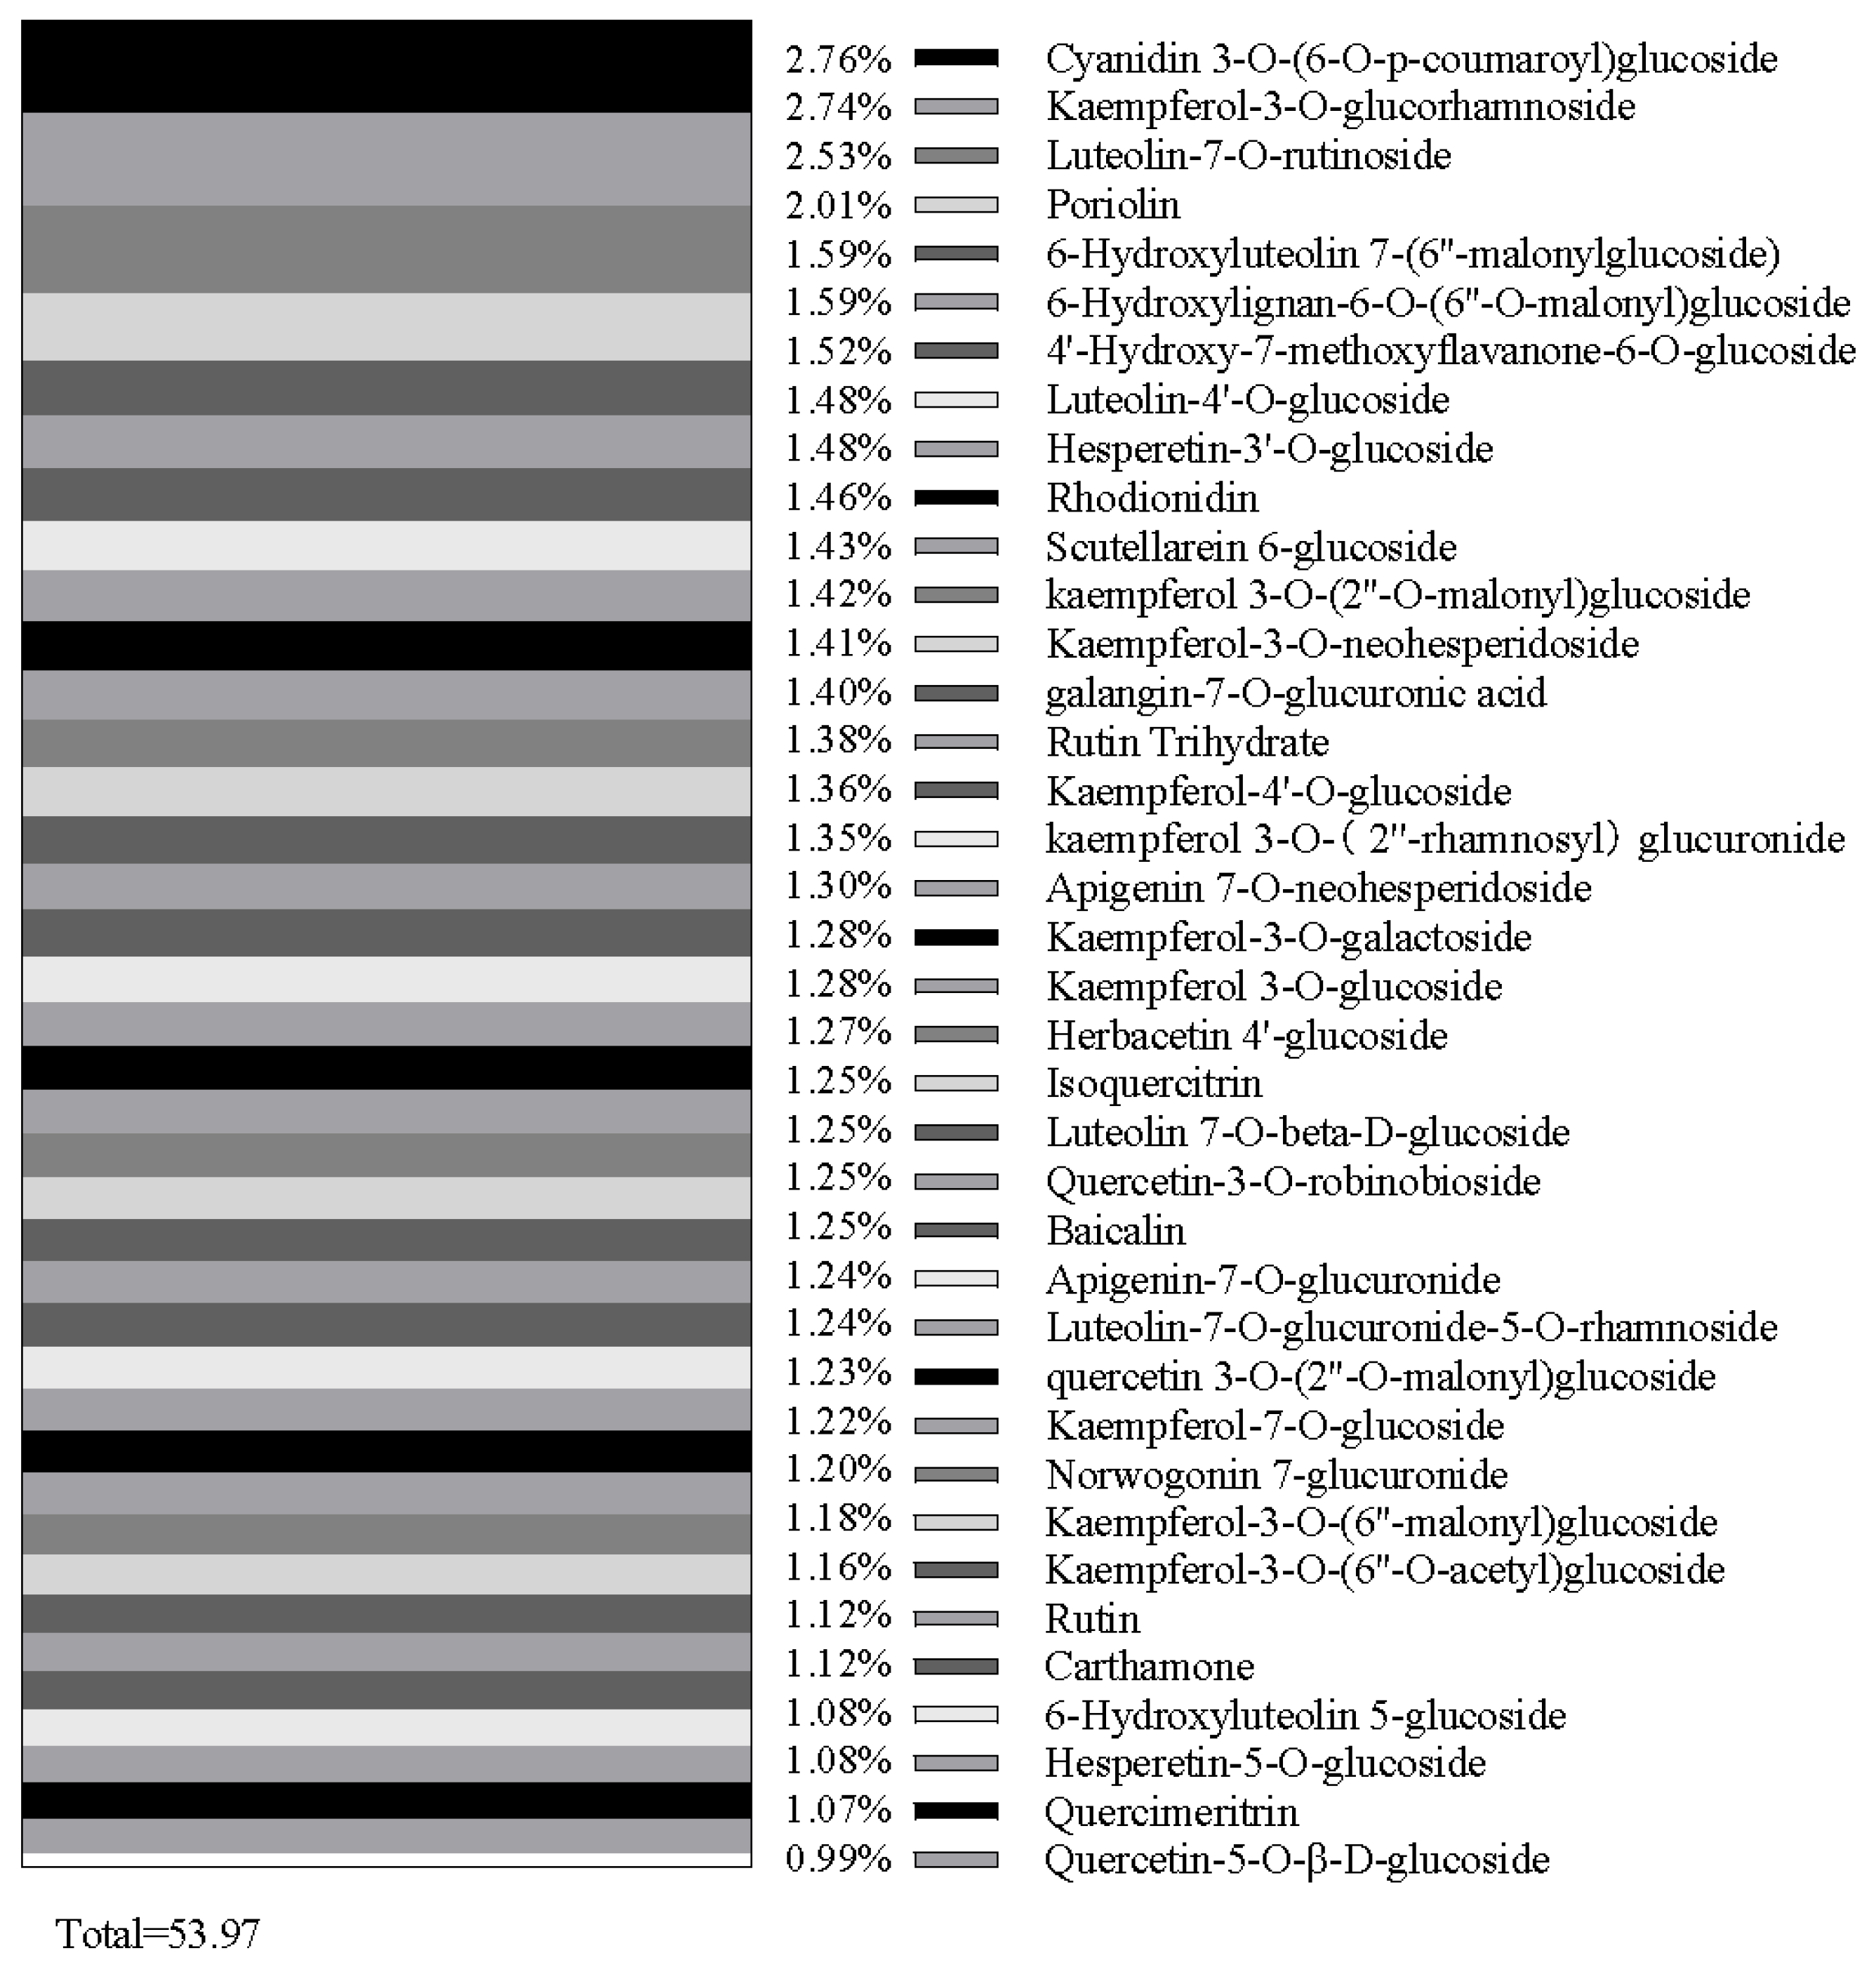
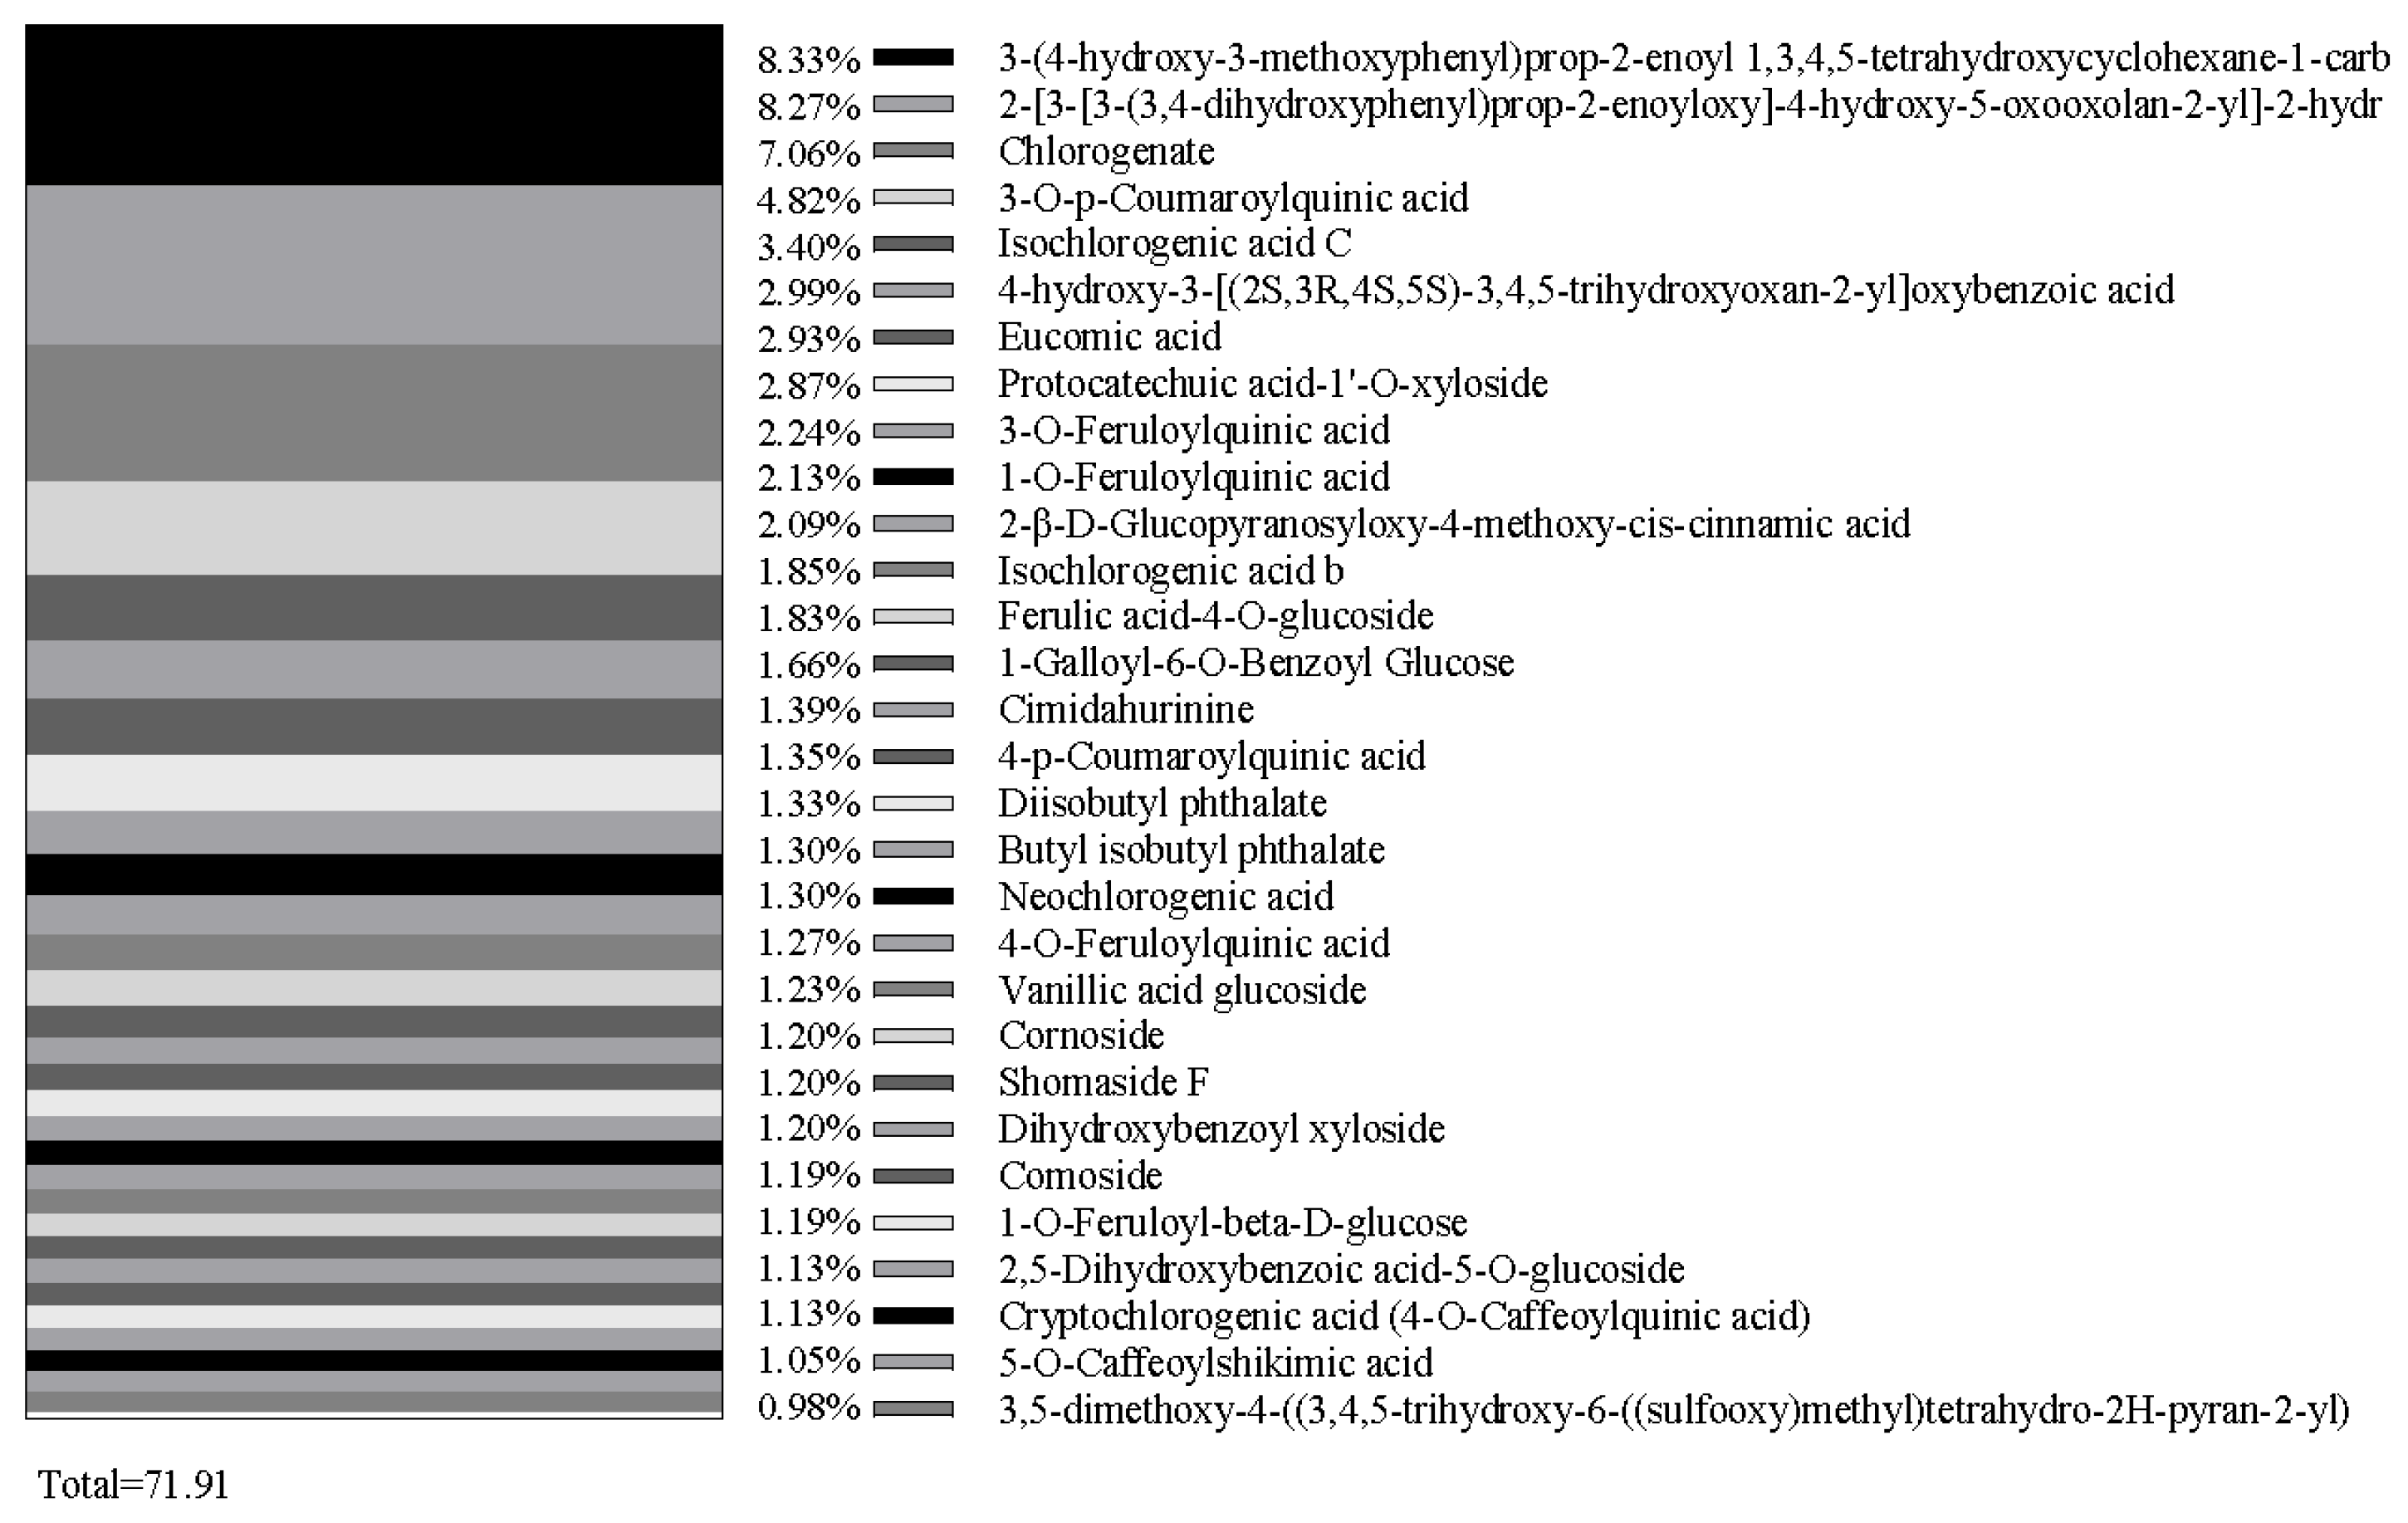
Flavonoids (65.41%) and phenolic acids (23.1%) collectively comprise 88.51% of all identified compounds resulting from the methanol extracts of C. vulgare leaves. Thirty major compounds, such as 3-(4-hydroxy-3-methoxyphenyl)prop-2-enoyl 1,3,4,5-tetrahydroxycyclohexane-1-carboxylate (2.17%), 2-[3-[3-(3,4-dihydroxyphenyl)prop-2-enoyloxy]-4-hydroxy-5-oxooxolan-2-yl]-2-hydroxyacetic acid (2.16%), cyanidin 3-O-(6-O-p-coumaroyl) glucoside (2.04%), kaempferol-3-O-glucorhamnoside (2.02%), luteolin-7-O-rutinoside (1.87%), and chlorogenate (1.84%), from flavonoids and phenolic acids, were selected (Figure 1 and Table 5). Moreover, thirty-eight flavonoid compounds and thirty phenolic acid compounds occupied by near and over 1.0% of content were selected, representing 53.97% and 71.91% of the total content of flavonoids and phenolic acids, respectively (Figure 2 and Figure 3). Many compounds of these flavonoids and phenolic acids are known allelochemicals produced by other plant species and their phytotoxic effects have been previously reported.
Figure 1.
Total ions current chromatogram (by UPLC-MS) of some main phenolic acid and flavonoid compounds from methanol extracts of Cirsium vulgare.
Table 5.
Main phenolic acid and flavonoid compounds of methanol extracts of Cirsium vulgare.
Figure 2.
Main flavonoid compounds of methanol extracts of Cirsium vulgare.
Figure 3.
Main phenolic acid compounds of methanol extracts of Cirsium vulgare.
3. Discussion
The current study demonstrated that aqueous extracts of C. vulgare exhibited phytotoxic activity, significantly inhibiting seed germination and seedling growth of B. pilosa and D. sanguinalis. Increasing numbers of studies have indicated that allelopathy is one of the main drivers for biological invasions and many invasive plant species can inhibit growth of neighboring plants via allelopathy [6,10,28,29]. However, with C. vulgare being a newly reported invasive plant species for Yunnan Province, China, its potential allelochemicals and its allelopathic effects on neighboring plants were unknown prior to the present study.
This study showed that the phytotoxic effects of aqueous extracts of C. vulgare increased with increasing extract concentration, which was consistent with many other research studies [10,30,31]. There were obvious differences in species-specific growth inhibitory activities from the various plant extracts. Inhibitory rates were generally higher for extracts from flower/fruit heads and leaves compared to stems, with the lowest rates of inhibition observed for roots, suggesting that the presence of phytotoxic substances may be richer in leaves and flower/fruit heads than in roots. Other studies have also shown that above-ground parts have greater allelopathic effects than other parts [10,32,33]. Fernandez et al. [33] reported that the leaves of Pinus halepensis Mill. (Pinaceae) contained higher levels and a greater variety of allelochemical compounds compared to its roots. Shen et al. [10] found that the invasive plant Acmella radicans (Jacq.) R.K.Jansen (Asteraceae) had allelopathic potential on Brassica rapa L. (Brassicaceae) and Chrysanthemum coronarium L. (Asteraceae) (now known as Glebionis coronaria (L.) Cass. ex Spach), with the overall inhibition rates ranked in the order flower/fruit head > leaf > stem > root.
Flavonoids (65.41%) and phenolic acids (23.1%) accounted for 88.51% of all identified compounds in the methanol extracts of C. vulgare in this study. Thirty-eight major flavonoid compounds and thirty major phenolic acid compounds were selected, representing 53.97% and 71.91% of the total content of flavonoids and phenolic acids, respectively. Many compounds of these flavonoids and phenolic acids such as ferulic acid [26], vanillic acid [30], proline [34], rutin [35], apigenin [36], luteolin [37], quercetin [38], kaempferol [39], isochlorogenic acid [40], and protocatechuic acid [41] have been previously reported to be known allelochemicals and have possible allelopathic effects. However, the phytotoxic potential of some compounds identified from the methanol extracts of C. vulgare still remains unclear and requires further investigation.
Allelopathic compounds can be released at any time during the life cycle of plants under natural conditions, but the allelopathic potential of different plant parts under different extraction methods varies greatly [42,43]. Some previous studies have shown that C. vulgare contains phenolic acid and flavonoid compounds and has strong antioxidant activity, but this depends on plant part and extraction method. Kozyra and Głowniak [20] found that the methanol extracts from dried flowering herbs of C. vulgare have richer phenolic acids and higher content compared to the water extracts from the leaves [22]. The highest total flavonoid content from whole plant parts of C. vulgare was found using methanol extracts, followed by ethyl acetate and diethyl ether extracts, while no flavonoids were found from hexane extracts [25]. Moreover, the highest yield of phenolic compounds from dried leaves of C. vulgare was produced by heat-reflux extraction for 90 min using 50% ethanol as a solvent [44]. Different phenolic compounds were obtained from various petrol, chloroform, and methanolic extracts of C. vulgare dried flower heads [45]. The methanolic and aqueous extracts and fractions of dried inflorescences and leaves of C. vulgare generally showed antioxidant and antimicrobial activity, which depends on phenolic compounds [19,21,22,45]. The current study found that there are abundant phenolic acid and flavonoid compounds in fresh leaves of C. vulgare for its phytotoxic effects, although they may differ between various plant parts and with different extraction methods.
Currently, C. vulgare is seen as an emerging serious invasive plant and most populations are distributed in Central Yunnan Province, China. In a separate modeling study, MaxEnt analysis showed that the potential suitable area of C. vulgare in China is predominantly concentrated in the northwest, southwest, and central regions of the mainland, as well as Taiwan. From field observations, this species is well-adapted to urban environments and is commonly found in green areas such as parks, flower beds, wastelands, and roadsides across cities and suburbs. Cirsium vulgare usually exhibits a competitive advantage in plant communities due to its high plant height, broad leaves, deep root system, and injurious spines. The present study showed that C. vulgare has strong allelopathic potential against seed germination and seedling growth of two common weeds in Yunnan Province through releasing phenolic acid and flavonoid compounds. These were primarily released in leaf and flower/fruit head leachates. The strong allelopathic potential of C. vulgare against B. pilosa and D. sanguinalis suggests that its management strategies must account for chemical interference, not merely resource competition. Therefore, in order to reduce both seed dispersal and allelochemicals inputs into the soil, early removal of above-ground biomass and plant residues of C. vulgare should be considered. In addition, applications of the phytotoxicity of C. vulgare could be explored such as in suppressing neighboring weed species or developing novel, plant-derived weed management tools.
4. Materials and Methods
4.1. Plant Materials Collection
Cirsium vulgare is biennial, and occasionally behaves as an annual under favorable conditions. It is widely distributed in Kunming City of Yunnan Province of China. Whole plants of C. vulgare were collected during the flowering and fruiting period in green belts of Yunnan Academy of Agricultural Sciences, China in June 2024. After harvesting, fresh plant samples were divided into four groups (roots, stems, leaves, and flower/fruit heads) and then cut into pieces (approximately 1–2 mm) for aqueous extraction and bioassay.
4.2. Test Plant Species, Aqueous Extract Preparation, and Bioassay
Two test species, B. pilosa and D. sanguinalis were used for biological assay. Bidens pilosa and D. sanguinalis are noxious weeds and commonly occur in temperate, subtropical, and tropical regions in Yunnan Province.
The extracts of roots, stems, leaves, and flower/fruit heads of C. vulgare were all prepared using the same method: 50 g of fresh tissue segments was immersed in 500 mL of distilled water (10% w/v) at room temperature (20 ± 5 °C). The extracts were stored in a refrigerator for 48 h before filtering. Filtration was performed by first passing the extracts through two layers of cheesecloth and then through two layers of filter paper. The filtered aqueous extracts had an initial concentration of 0.1 g·mL−1. For subsequent bioassays, the extracts were then diluted with distilled water to four concentrations (0.0125, 0.025, 0.05, and 0.1 g·mL−1), as established in pre-experimental trials. The extract concentrations were relative low compared to some similar studies in which aqueous extracts from dried or fresh materials were prepared [10,32,33]. All solutions were stored at 4 °C until use.
To evaluate the allelopathic effects of C. vulgare on the two test species, the four extract concentrations and a control (distilled water, CK) were tested, each with four replicates. Twenty surface-sterilized seeds of each test species were evenly placed in separate Petri dishes (9 cm diameter) containing two layers of filter paper, and 5 mL of extract or distilled water (control) were added in each treatment. The bioassay procedures for assessing the effects of the different concentrations on the germination of seeds and biomass of seedlings of the two plant species were identical to those described by Shen et al. [46]. Germination counts were made daily, while shoot height, root length, and seedling fresh biomass were determined after the 7-day experimental period.
4.3. Identification of Flavonoid and Phenolic Compounds
Based on initial bioassay analysis and previous studies on phenolic acid and flavonoid compounds of C. vulgare [20,22,25], leaves were selected for further study using the methanol extract method. The young fresh leaves of C. vulgare were collected and placed in a lyophilizer (Scientz-100F, Scientz, Ningbo, China) for 63 h, then ground (30 Hz, 1.5 min) to powder form using a grinder (MM 400, Retsch, Haan, Germany). Then, 30 mg of sample powder was weighed using an electronic balance (MS105DΜ) and 1500 μL of −20 °C pre-cooled 70% methanol aqueous internal standard extract (less than 30 mg added at the rate of 1500 μL extractant per 30 mg sample) was added. The samples were placed in a Vortex once every 30 min for 30 s, for a total of 6 times. After centrifugation (rotation speed 12,000 rpm, 3 min), the supernatant was aspirated, and the sample was filtered through a microporous membrane (0.22 μm pore size) and stored in the injection vial for UPLC-MS/MS analysis.
4.4. UPLC-MS Analysis
The sample extracts were analyzed using an ultraperformance liquid chromatography−electrospray ionization tandem mass spectrometry (UPLC-ESI-MS/MS). The analytical conditions of UPLC were as follows: Column, Agilent SB-C18 (1.8 µm, 2.1 mm × 100 mm; Agilent, Santa Clara, CA, USA). The mobile phase consisted of solvent A (pure water with 0.1% formic acid) and solvent B (acetonitrile with 0.1% formic acid). Sample measurements were performed with a gradient program that employed starting conditions of 95% A, 5% B. Within 9 min, a linear gradient to 5% A, 95% B was programmed, and a composition of 5% A, 95% B was kept for 1 min. Subsequently, a composition of 95% A, 5.0% B was adjusted within 1.1 min and kept for 2.9 min. The flow velocity was set as 0.35 mL per minute, the column oven was set to 40 °C, and the injection volume was 2 μL. The effluent was alternatively connected to an ESI−triple quadrupole−linear ion trap (QTRAP)-MS.
The MS conditions were as follows: the source operation parameters of electrospray ionization (ESI) included source temperature 500 °C, ion spray voltage (IS) 5500 V (positive ion mode)/−4500 V (negative ion mode), ion source gas I (GSI) (50 psi), gas II (GSII) (60 psi), curtain gas (CUR) (25 psi), and high collision-activated dissociation (CAD). The triple quadrupole (QQQ) scans were acquired as multiple reaction monitoring (MRM) experiments with collision gas (nitrogen) set to medium. The declustering potential (DP) and collision energy (CE) for individual MRM transitions were done with further DP and CE optimization. A specific set of MRM transitions was monitored for each period according to the metabolites eluted within this period.
Metabolite identification was performed using secondary mass spectral data. After obtaining the mass spectrometry data of metabolites from different samples, peak area integration was conducted for all substance chromatographic peaks, and integration correction was applied for the same metabolite detected across different samples [47].
4.5. Statistical Analysis
Data were analyzed using IBM SPSS software version 23.0 (Armonk, New York, NY, USA). The inhibitory rates (IRs) of aqueous extracts of C. vulgare for germination rate, germination index, plant height, and biomass were calculated using the formula (C − T)/C × 100%, where C is the mean value of control, and T is the mean value of each extract treatment (IR > 0 indicates inhibition, IR < 0 indicates promotion, and the magnitude of IR values reflects the intensity of the allelopathic effect) [48]. The allelopathic response index (RI) was calculated for aqueous extracts from B. pilosa and D. sanguinalis. The formula for RI is: when T ≥ C, RI = 1 − C/T; when T < C, RI = T/C − 1, where C is the control value and T is the treatment value; R > 0 indicates promotion, IR < 0 indicates inhibition, and the magnitude of IR values reflects the intensity of the allelopathic effect [49]. A synthetical allelopathic index was then derived by averaging the RI values obtained for germination rate, germination index, root length, shoot length, and biomass. The result data were analyzed using two-way ANOVA to evaluate plant part and concentration levels, with their interaction (ns, *, and ** indicate p > 0.05, p ≤ 0.05, and p ≤ 0.01, respectively, for F value), and one-way ANOVA to evaluate inhibitory rate and allelopathic response index (5% significance level). Duncan’s multiple range tests were conducted to compare treatment differences (p < 0.05) for significant differences detected by ANOVA.
5. Conclusions
This study showed that extracts of C. vulgare inhibited the growth of B. pilosa and D. sanguinalis. The inhibitory rates of the aqueous extracts of C. vulgare on seed germination and seedling growth of B. pilosa were generally higher than the rates for D. sanguinalis. The germination rate, germination index, root length, shoot length, and biomass of the two test species significantly declined as the concentration of C. vulgare extracts increased. Comparing the allelopathic response indices derived from the four aqueous extracts of C. vulgare on B. pilosa and D. sanguinalis, flower/fruit heads and leaves yielded the strongest inhibition, followed by stems, with the lowest impact from root extracts. Thirty-eight major flavonoid and thirty major phenolic acids were identified from the methanol extracts of C. vulgare, with many compounds, including ferulic acid, vanillic acid, proline, rutin, apigenin, luteolin, quercetin, kaempferol, isochlorogenic acid, and protocatechuic acid having been reported to have possible allelopathic effects and considered as potential allelochemicals in previous research. However, the phytotoxic potential of some compounds from the methanol extracts of C. vulgare is still not clear and needs to be further tested, although phenolic compounds have been considered as potential allelochemicals. Therefore, complementary field-based studies and further studies on the allelochemicals and allelopathic mechanisms of C. vulgare under various conditions would provide valuable additional information on how the allelopathic potential of C. vulgare facilitates its invasiveness.
Author Contributions
F.Z. (Fengping Zheng): investigation; writing—original draft. C.Z.: data curation; writing—original draft. K.Y.: data curation; investigation. Q.L.: investigation. Z.W.: investigation. G.X.: investigation. D.R.C.: conceptualization; writing—review and editing. B.Y.: investigation. G.J.: investigation. S.Y.: investigation. F.Z. (Fudou Zhang): conceptualization; project administration. M.D.D.: writing—review and editing. S.S.: conceptualization; data curation; funding acquisition; investigation; project administration; supervision; writing—original draft. All authors have read and agreed to the published version of the manuscript.
Funding
This research was supported by the National Key Research and Development Program of China (2024YFC2607600), Yunnan Fundamental Research Project (202501AS070027), Yunnan Provincial Agricultural Basic Research Joint Special Project (202401BD070001-019), National Natural Science Foundation of China (31960569), Key Research and Development Program of Yunnan Province (202103AF140007, 202203AE140008), and Ten Thousand Talent Program (Young Top-Notch Talent) of Yunnan Province (YNWR-QNBJ-2018-201).
Data Availability Statement
The original contributions presented in this study are included in the article. Further inquiries can be directed to the corresponding author(s).
Acknowledgments
We wish to thank Xiaohan Wu, from the School of Agriculture, Yunnan University, for her great field support.
Conflicts of Interest
The authors declare no conflicts of interest. The founding sponsors had no role in the design of the study; in the collection, analyses, or interpretation of data; in the writing of the manuscript, and in the decision to publish the results.
References
- Rai, P.K.; Singh, J.S. Invasive alien plant species: Their impact on environment, ecosystem services and human health. Ecol. Indic. 2020, 111, 106020. [Google Scholar] [CrossRef] [Scilit]
- Diagne, C.; Leroy, B.; Vaissière, A.C.; Gozlan, R.E.; Roiz, D.; Jarić, I.; Salles, J.M.; Bradshaw, C.J.A.; Courchamp, F. High and rising economic costs of biological invasions worldwide. Nature 2021, 592, 571–576. [Google Scholar] [CrossRef] [Scilit]
- Vilà, M.; Espinar, J.L.; Hejda, M.; Hulme, P.E.; Jarošík, V.; Maron, J.L.; Pergl, J.; Schaffner, U.; Sun, Y.; Pyšek, P. Ecological impacts of invasive alien plants: A meta-analysis of their effects on species, communities and ecosystems. Ecol. Lett. 2011, 14, 702–708. [Google Scholar] [CrossRef] [Scilit]
- Li, F.; Hao, Q.; Cui, X.; Lin, R.; Luo, B.; Ma, S. Global invasive alien plant management lists: Assessing current practices and adapting to new demands. Plant Divers. 2025, 47, 666–680. [Google Scholar] [CrossRef] [Scilit]
- Kalisz, S.; Kivlin, S.N.; Bialic-Murphy, L. Allelopathy is pervasive in invasive plants. Biol. Invasions 2021, 23, 367–371. [Google Scholar] [CrossRef] [Scilit]
- Batish, D.; Singh, H.; Kaur, S.; Kohli, R.; Jose, S. Novel Weapon Hypothesis for the Successful Establishment of Invasive Plants in Alien Environments. In Invasive Plant Ecology; Jose, S., Singh, H.P., Batish, D.R., Kohli, R.K., Eds.; CRC Press: Boca Raton, FL, USA, 2013; pp. 19–28. [Google Scholar]
- Shen, S.; Xu, G.; Li, D.; Yang, S.; Jin, G.; Liu, S.; Clements, D.R.; Chen, A.; Zhang, F.; Wen, L.; et al. Adventitious roots support population expansion of the invasive plant Mikania micrantha Kunth. Physiol. Plantarum 2021, 173, 911–919. [Google Scholar] [CrossRef] [Scilit]
- Guo, K.; Pyšek, P.; van Kleunen, M.; Kinlock, N.L.; Lučanová, M.; Leitch, I.J.; Pierce, S.; Dawson, W.; Essl, F.; Kreft, H.; et al. Plant invasion and naturalization are influenced by genome size, ecology and economic use globally. Nat. Commun. 2024, 15, 1330. [Google Scholar] [CrossRef] [Scilit]
- Peng, S.; Chen, Z.; Wen, J.; Shao, H. Is allelopathy a driving force in forest succession? Allelopath. J. 2004, 14, 197–204. [Google Scholar]
- Shen, S.; Xu, G.; Yang, S.; Jin, G.; Clements, D.R.; Yang, K.; Wu, X.; Fan, Z.; Zhang, F. How do the extracts from the invasive plant Acmella radicans inhibit germination and growth of Brassica rapa (field mustard) and Chrysanthemum coronarium (garland daisy)? Int. J. Agron. 2025, 2025, 8270456. [Google Scholar] [CrossRef] [Scilit]
- Meusel, H.; Jäger, E.J. Vergleichende Chorologie der Zentraleuropäischen Flora; Gustav Fischer: Jena, Germany; Stuttgart, Germany; New York, NY, USA, 1992; Volume 3. [Google Scholar]
- Klinkhamer, P.G.L.; De Jong, T.J. Cirsium vulgare (Savi) Ten. J. Ecol. 1993, 81, 177–191. [Google Scholar] [CrossRef] [Scilit]
- Bureš, P.; Guacchio, E.D.; Šmerda, J.; Özcan, M.; Blizňáková, P.; Vavrinec, M.; Michálková, E.; Veselý, P.; Veselá, K.; Zedek, F. Intergeneric hybrid origin of the invasive tetraploid Cirsium vulgare. Plant Biol. 2024, 26, 749–763. [Google Scholar] [CrossRef] [Scilit]
- Forcella, F.; Wood, H. Demography and control of Cirsium vulgare (Savi) Ten. in relation to grazing. Weed Res. 1986, 26, 199–206. [Google Scholar] [CrossRef] [Scilit]
- Parsons, W.T.; Cuthbertson, E.G. Noxious Weeds of Australia, 2nd ed.; CSIRO Publishing: Collingwood, VIC, Australia, 2001. [Google Scholar]
- Román, J.F.C.; Hernán dez-Lambraño, R.E.; Rodríguez de la Cruz, D.; Sánchez Agudo, J.Á. Analysis of the adaptative strategy of Cirsium vulgare (Savi) Ten. in the colonization of new territories. Sustainability 2021, 13, 2384. [Google Scholar] [CrossRef] [Scilit]
- Iwashina, T.; Kadota, Y.; Ueno, T.; Ootani, S. Foliar flavonoid composition in Japanese Cirsium species (Compositae), and their chemotaxonomic significance. J. Jpn. Bot. 1995, 70, 280–290. [Google Scholar]
- Jordon-Thaden, I.E.; Louda, S.M. Chemistry of Cirsium and Carduus: A role in ecological risk assessment for biological control of weeds? Biochem. Syst. Ecol. 2003, 31, 1353–1396. [Google Scholar] [CrossRef] [Scilit]
- Nazaruk, J.; Jakoniuk, P. Flavonoid composition and antimicrobial activity of Cirsium rivulare (Jacq.) All. flowers. J. Ethnopharmacol. 2005, 102, 208–212. [Google Scholar] [CrossRef] [Scilit]
- Kozyra, M.; Głowniak, K. Phenolic acids in extracts obtained from the flowering herbs of Cirsium vulgare (Savi) Ten. growing in Poland. Acta Soc. Bot. Pol. 2013, 82, 325–329. [Google Scholar] [CrossRef] [Scilit]
- Nazaruk, J. Antioxidant activity and total phenolic content in Cirsium five species from north-east region of Poland. Fitoterapia 2008, 79, 194–196. [Google Scholar] [CrossRef] [Scilit]
- Nazaruk, J.; Czechowska, S.K.; Markiewicz, R.; Borawska, M.H. Polyphenolic compounds and in vitro antimicrobial and antioxidant activity of aqueous extracts from leaves of some Cirsium species. Nat. Prod. Res. 2008, 22, 1583–1588. [Google Scholar] [CrossRef] [Scilit]
- Yin, J.; Heo, S.I.; Wang, M. Antioxidant and antidiabetic activities of extracts from Cirsium japonicum roots. Nutr. Res. Pract. 2008, 2, 247–251. [Google Scholar] [CrossRef] [Scilit]
- Hoang Anh, L.; Van Quan, N.; Tuan Nghia, L.; Dang Xuan, T. Phenolic allelochemicals: Achievements, limitations, and prospective approaches in weed management. Weed Biol. Manag. 2021, 21, 37–67. [Google Scholar] [CrossRef] [Scilit]
- Aydın Kurç, M.; Orak, H.H.; Gülen, D.; Caliskan, H.; Argon, M.; Sabudak, T. Antimicrobial and antioxidant efficacy of the lipophilic extract of Cirsium vulgare. Molecules 2023, 28, 7177. [Google Scholar] [CrossRef] [Scilit]
- Mushtaq, W.; Fauconnier, M.L. Phenolic profiling unravelling allelopathic encounters in agroecology. Plant Stress. 2024, 13, 100523. [Google Scholar] [CrossRef] [Scilit]
- Kumar, N.; Singh, H.; Giri, K.; Kumar, A.; Joshi, A.; Yadav, S.; Mishra, G. Physiological and molecular insights into the allelopathic effects on agroecosystems under changing environmental conditions. Physiol. Mol. Biol. Pla. 2024, 30, 417–433. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, T.; Liu, W.; Zhang, C.; Wang, J. Effects of Solidago canadensis invasion on dynamics of native plant communities and their mechanisms. Chin. J. Plant Ecol. 2012, 36, 253–261. [Google Scholar] [CrossRef] [Scilit]
- Yang, K.; Yang, Y.; Wu, X.; Zheng, F.; Xu, G.; Yang, S.; Jin, G.; Clements, D.R.; Shen, S.; Zhang, F. Allelopathic potential and chemical composition of essential oil from the invasive plant Acmella radicans. Agronomy 2024, 14, 342. [Google Scholar] [CrossRef] [Scilit]
- Hossen, K.; Das, K.R.; Okada, S.; Iwasaki, A.; Suenaga, K.; Kato-Noguchi, H. Allelopathic potential and active substances from Wedelia chinensis (Osbeck). Foods 2020, 9, 1591. [Google Scholar] [CrossRef] [Scilit]
- Boonmee, S.; Iwasaki, A.; Suenaga, K.; Kato-Noguchi, H. Evaluation of phytotoxic activity of leaf and stem extracts and identification of a phytotoxic substance from Caesalpinia mimosoides Lamk. Theor. Exp. Plant Phys. 2018, 30, 129–139. [Google Scholar] [CrossRef] [Scilit]
- Abdelmalik, A.M.; Alshahrani, T.S.; Alqarawi, A.A.; Ahmed, E.M. Allelopathic potential of Nicotiana glauca aqueous extract on seed germination and seedlings of Acacia gerrardii. Diversity 2023, 16, 26. [Google Scholar] [CrossRef] [Scilit]
- Fernandez, C.; Monnier, Y.; Ormeño, E.; Baldy, V.; Greff, S.; Pasqualini, V.; Mévy, J.P.; Bousquet-Mélou, A. Variations in allelochemical composition of leachates of different organs and maturity stages of Pinus halepensis. J. Chem. Ecol. 2009, 35, 970–979. [Google Scholar] [CrossRef] [Scilit]
- Al Musalami, A.A.; Al Marshoudi, M.S.; Farooq, S.A.; Al-Reasi, H.A. Allelopathic effects of the invasive species (Prosopis juliflora) on seedlings of two common arid plants: Does free proline play roles? J. Arid. Environ. 2023, 211, 104931. [Google Scholar] [CrossRef] [Scilit]
- Averett, J.E.; Banks, W.A.; Boehme, D.E. Negative allelopathic effects of rutin and quercetin on fourteen soil and enteric microbes. Biochem. Syst. Ecol. 1978, 6, 1–3. [Google Scholar] [CrossRef] [Scilit]
- Szwed, M.; Mitrus, J.; Wiczkowski, W.; Dębski, H.; Horbowicz, M. The allelopathic properties of decomposing buckwheat residues are not directly related to phenolic compounds in soil. Plant Soil. Environ. 2020, 66, 200–206. [Google Scholar] [CrossRef] [Scilit]
- Cao, L.; Li, J. Plant-originated kaempferol and luteolin as allelopathic algaecides inhibit aquatic microcystis growth through affecting cell damage, photosynthetic and antioxidant responses. J. Biodegradat. Bioremed. 2018, 9, 431. [Google Scholar] [CrossRef]
- Fernández-Aparicio, M.; Masi, M.; Cimmino, A.; Vilariño, S.; Evidente, A. Allelopathic effect of quercetin, a flavonoid from Fagopyrum esculentum roots in the radicle growth of Phelipanche ramosa: Quercetin natural and semisynthetic analogues were used for a structure-activity relationship investigation. Plants 2021, 10, 543. [Google Scholar] [CrossRef] [Scilit]
- Kong, F.; Zhao, Q.; Wen, W.; He, P.; Shao, L. Allelopathic effects and mechanism of kaempferol on controlling Microcystis aeruginosa blooms. Mar. Pollut. Bull. 2025, 217, 118116. [Google Scholar] [CrossRef] [Scilit]
- Chen, L.; Li, J.; Zhu, Y.; Zhao, T.; Guo, L.; Kang, L.; Yu, J.; Du, H.; Liu, D. Weed suppression and molecular mechanisms of isochlorogenic acid A isolated from Artemisia argyi extract via an activity-guided method. J. Agric. Food Chem. 2022, 70, 1494–1506. [Google Scholar] [CrossRef] [Scilit]
- Chen, Q.; Zhu, B.; Sun, D.; Liu, W.; Sun, X.; Duan, S. The effect of protocatechuic acid on the phycosphere in harmful algal bloom species Scrippsiella trochoidea. Aquat. Toxicol. 2020, 227, 105591. [Google Scholar] [CrossRef] [Scilit]
- Ma, G.; Xu, G.; Yang, S.; Yang, Y.; Zhang, F.; Wen, L.; Tao, Q.; Shen, S.; Ye, M. Allelopathy of sweet potato (Ipomoea batatas) extracts on seed germination and seedling growth of three weeds. Southwest. China J. Agr. Sci. 2022, 35, 1295–1302. [Google Scholar] [CrossRef]
- Clavijo McCormick, A.; Efah, E.; Najar-Rodriguez, A. Ecological aspects of volatile organic compounds emitted by exotic invasive plants. Front. Ecol. Evol. 2023, 11, 1059125. [Google Scholar] [CrossRef] [Scilit]
- Griškevičienė, U.; Marksa, M.; Ževžikovienė, A.; Kazlauskienė, D.R.; Vainorienė, R.; Ževžikovas, A.; Ivanauskas, L. Cirsium vulgare leaves: Isolation and identification of phenolic compounds. Chemija 2021, 32, 92–99. [Google Scholar] [CrossRef] [Scilit]
- Nazaruk, J.; Chłędzik, S.; Strawa, J.; Bazydło, K.; Wajs-Bonikowska, A. Chemical composition and antioxidant activity of Cirsium vulgare (Savi) Ten. inflorescences. Nat. Prod. Commun. 2017, 12, 519–522. [Google Scholar] [CrossRef] [Scilit]
- Shen, S.; Xu, G.; Li, D.; Clements, D.R.; Jin, G.; Liu, S.; Yang, Y.; Chen, A.; Zhang, F.; Kato-Noguchi, H. Allelopathic potential of sweet potato (Ipomoea batatas) germplasm resources of Yunnan Province in southwest China. Acta Ecol. Sin. 2018, 38, 444–449. [Google Scholar] [CrossRef] [Scilit]
- Fraga, C.G.; Clowers, B.H.; Moore, R.J.; Zink, E.M. Signature-discovery approach for sample matching of a nerve-agent precursor using liquid chromatography-mass spectrometry, XCMS, and chemometrics. Anal. Chem. 2010, 82, 4165–4173. [Google Scholar] [CrossRef] [Scilit]
- Li, X.; Wang, J.; Huang, D.; Wang, L.; Wang, K. Allelopathic potential of Artemisia frigida and successional changes of plant communities in the northern China steppe. Plant Soil. 2011, 341, 383–398. [Google Scholar] [CrossRef] [Scilit]
- Bruce Williamson, G.; Richardson, D. Bioassays for allelopathy: Measuring treatment responses with independent controls. J. Chem. Ecol. 1998, 14, 181–187. [Google Scholar] [CrossRef] [Scilit] [PubMed]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.