


Abstract
While water content is a critical factor affecting the outcome of cryopreservation, the mechanism by which it influences seed viability after cryopreservation remains unclear. In this study, Paeonia lactiflora seeds with different water content as experimental materials, analyzed the seed viability, oxidative stress indicators, and transcriptomics before and after cryopreservation, to explore the mechanism of the seed viability changes. The results demonstrated that after cryopreservation, seeds with high water content displayed reduced viability, along with abnormal accumulation of reactive oxygen species (ROS) content, which subsequently triggered ROS-mediated oxidative damage. In contrast, seeds with low water exhibited enhanced following cryopreservation, their ROS levels remained relatively stable, while notable alterations were detected in multiple antioxidant system parameters. At the transcriptional level, 1224 differentially expressed genes (DEGs) up-regulated and 1839 DEGs were down-regulated in seeds with high water content after cryopreservation, but 2090 DEGs up-regulated and 1783 DEGs down-regulated in the seeds with low water content. Among them, 687 DEGs were common to both the high- and low-water content seed groups. Gene Ontology (GO) functional analysis indicated that these DEGs are primarily involved physiological metabolic processes including osmotic response, glucosidase activity, protein kinase binding, and response to hydrogen peroxide. Kyoto Encyclopedia of Genes and Genomes (KEGG) pathway enrichment analysis confirmed that the Mitogen-Activated Protein Kinase (MAKP) plant signaling pathway and the starch and sucrose metabolism pathway are the key pathways governing the response of seeds with varying water contents to cryopreservation. Finally, through weighted gene co-expression network pinpointed DHN1 and LEA34 as the core genes regulating changes in seed viability after cryopreservation. These findings offer a broader perspective for in-depth exploration of the molecular regulatory mechanisms underlying the differences in seed viability changes after cryopreservation and are crucial for comprehensively clarifying the precise pathways via which these key genes regulate seed viability changes after cryopreservation.
1. Introduction
Seeds are important plant genetic resources, carrying all the genetic material required for development. As the foundation of plant breeding, seeds are one of the main materials for the preservation of plant germplasm resources due to their small size and portability [1]. Cryopreservation, a technology of preserving biological materials at liquid nitrogen (LN, −196 °C) or liquid nitrogen vapor (−168 °C), inhibits the physiological metabolic activities of plant materials and reduces the rate of deterioration [2,3]. Compared with traditional seed preservation methods, cryopreservation is currently the most promising method for long-term preservation of germplasm resources. Cryopreservation integrates simplicity, safety, and energy efficiency, and has yielded promising results in preserving the seeds of numerous plant species [4,5]. However, some species cannot be preserved by cryopreservation or their viability is significantly decreased after cryopreservation.
Since the widespread application of cryopreservation technology in plant germplasm conservation during the 1980s, researchers conducted extensive investigations into the phenomenon of viability decline after cryopreservation, and their findings indicate that the reasons are multifaceted. Among them, water content is extremely crucial. For different types of seeds, the optimal water content for cryopreservation varies. Before cryopreservation, the seeds need to be dried to the appropriate water content [6]. When the water content of the seeds is too low, it may cause excessive dehydration of the seeds, resulting in cell plasmolysis and deformation, an increase in the concentration of solutes in the intracellular and extracellular fluids, and deterioration of the biochemical environment within the cells [4]. When seeds with high water content are subjected to cryopreservation, during the freezing and rewarming process of cryopreservation, ice crystals form within the cells, damaging the cell membranes and disrupting the cell structure, and causing cell death [7]. Therefore, exploring the optimal seed water content not only ensures robust post-cryopreservation viability, but facilitates elucidation of the stress response mechanisms in seeds during cryopreservation [8].
Plant cells undergo various reactions leading to the excessive accumulation of reactive oxygen species (ROS) during cryopreservation, which disrupts the redox homeostasis within the cells. Then the overproduction of ROS results in severe damage to plant membrane lipids and proteinaceous substances, which causes viability decline after cryopreservation [9,10,11]. As a by-product of aerobic metabolism in plants, ROS are typically scavenged by antioxidant systems to maintain a balanced intracellular state, thus mitigating damage induced by ROS accumulation under stresses such as low temperature [12,13]. The antioxidant substances within plants that effectively scavenge ROS can be categorized into two primary types, enzymes, and non-enzymes antioxidants. The enzyme antioxidants primarily include superoxide dismutase (SOD), catalase (CAT), ascorbate peroxidase (APX), monodehydroascorbate reductase (MDHAR), glutathione reductase (GR), and dehydroascorbate reductase (DHAR) and others [14,15,16]. The non-enzymatic antioxidants mainly comprise substances such as ascorbic acid (AsA) and glutathione (GSH) [14,15,16]. The present literature has demonstrated that, whether through endogenous methods or exogenous means, antioxidant substances play an extremely significant role in viability changes in plant materials after cryopreservation. This phenomenon has been observed in the cryopreservation of blackberry (Rubus fruticosus) shoot tips, peony (Paeonia suffruticosa) and Chinese herbaceous peony (Paeonia lactiflora) pollen, rice (Oryza sativa) somatic embryos and arabidopsis (Arabidopsis thaliana) seedlings [9,10,11,17,18,19]. However, when the stress is intense, the antioxidant substances are unable to reduce the ROS components to within the controllable range. The highly accumulated ROS will trigger oxidative damage, such as increased lipid peroxidation levels of the cell membrane and protein denaturation [9,20]. Among the indicators, malondialdehyde (MDA) content and protein carbonyl (PCO) levels are commonly used to determine the degree of oxidative damage. Significant correlations have been documented between cell viability and MDA content during the cryopreservation of diverse plant materials, including somatic embryos of cacao (Theobroma cacao), embryogenic callus of African lily (Agapanthus praecox), shoot tips of blackberry (Rubus fruticosus), and pollen from 21 ornamental plant species [18,21,22,23]. In addition, there are also studies found that alterations in PCO levels serve as a critical determinant of cell viability changes after cryopreservation [11,24,25]. The existing research mostly focuses on the physiological level, and analyses of the mechanisms of viability changes in plant materials before and after cryopreservation.
Transcriptome sequencing is a high-throughput technique that allows for the rapid and comprehensive acquisition of nearly all transcripts and gene sequences from a specific cell or tissue of a given species under a particular state. It can be used to study gene expression levels, gene functions, and structures, as well as predict new transcripts, among other applications [26]. Up to now, the study of the mechanism underlying the changes in cell viability after cryopreservation using transcriptomics was relatively scarce in plants. The Hu et al. study based on transcriptome and physiological analysis revealed that the expression of the core gene PaMYB 11 played a crucial role in cell survival rates after cryopreservation in Norway spruce (Picea abies) embryogenic callus [27]. In addition, Htwe et al. discovered through RNA sequencing technology, the down-regulation of transferase activity of (glycan metabolism) genes related to maintaining the intracellular ROS balance and responding to osmotic and cold stress, which was the key factor affecting the cell survival rate of banana (Musa AAA cv Borjahaji) meristems after cryopreservation [28]. Ren et al. in their study on the cryopreservation of arabidopsis (A. thaliana) seedlings, based on the transcriptional level, revealed that the differential expression of genes related to the ROS metabolic system was one of the key reasons for the viability decline of the seedlings after cryopreservation [29]. Although limited transcriptional-level research has provided valuable theoretical references for innovation in cryopreservation technology, the current literature predominantly focuses on vitrification-cryopreservation techniques. These techniques not only involve extreme low-temperature stress, but also impose severe osmotic and cytotoxic stress. In contrast, cryopreservation of plant materials such as seeds using the direct freezing method is primarily challenged by extreme low temperatures during the process. Consequently, existing researchers were unable to directly demonstrate the impact of the cryopreservation process on cell viability.
The effective preservation of herbaceous peony (P. lactiflora) germplasm resources serves as the core foundation for its industrial upgrading and scientific research innovation. As a multi-purpose species, herbaceous peony (P. lactiflora) is not only a major cut flower crop but also possesses significant medicinal value [30,31]. In previous studies, our research group has investigated the cryopreservation technology and underlying mechanisms for herbaceous peony (P. lactiflora) pollen. However, pollen only carries the male genetic information of the species, whereas seeds harbor the complete genetic makeup of the organism, making them an ideal material for germplasm conservation. Although herbaceous peony (P. lactiflora) are produces intermediate seeds (seeds with desiccation tolerance and storage behavior between orthodox and recalcitrant seeds), their viability is highly susceptible to rapid decline. Therefore, this study used herbaceous peony (P. lactiflora) seeds with a range of water contents as experimental materials, employing the direct freezing method for cryopreservation. A comparative analysis was conducted to examine the differences in seed viability, ROS-induced oxidative stress levels, and transcriptional changes before and after cryopreservation. By integrating physiological and transcriptional data, this study explored the mechanisms of the differences in seed viability after cryopreservation based on the water content differences.
2. Materials and Methods
2.1. Plant Materials
The Chinese herbaceous peony (P. lactiflora) seeds used for the experiment were collected in August 2023 in Quwo County, Linfen City, Shanxi Province (111°50′ E, 35°66′ N). Thousand-grain weight is 281.17 g, the initial natural water content is 21.56%, and the seeds with water content of 4.35% were obtained through the silica gel weight reduction method [32].
Seed cryopreservation was carried out using the direct freezing method. The seeds with natural water content (21.56%, high-water content) and those after drying (4.35%, low-water content) were placed in 5 mL cryotubes, immersed directly into liquid nitrogen (LN, −196 °C) and held for at least seven days. After cryopreservation, the cryotubes containing seeds were thawed in running water for 10 min and then incubated in 20 °C water for 25 min to ensure complete thawing.
2.2. Determination of Seed Viability
Seed germination rate was determined via the sand storage method [32]. In mid-October (autumn), seeds were soaked for 12 h and subsequently placed in moistened fine sand under outdoor conditions. Germination status was recorded in spring (mid-March) of the following year. Each water content gradient was tested in triplicate, and the results were averaged.
Seed viability determination was carried out using the 2,3,5-triphenyltetrazolium chloride staining method repeated three times [32]. The detailed measurement procedures for all indicators can be found in previous research [33].
2.3. Determination of Oxidative Stress Indicators in Seeds
Superoxide anion free radical (O2·−) was determined via the hydroxylamine oxidation method [34]. Hydrogen peroxide (H2O2) and hydroxyl radical (·OH) contents were measured using commercial kits from Nanjing Jiancheng Bioengineering Institute, with the corresponding kit catalog numbers being A064-1-1 and A018-1-1, respectively. Malondialdehyde (MDA) content was assayed via the thiobarbituric acid method [23], while protein carbonyl (PCO) content was determined as described by Gogorcena et al. (1995) [35]. Superoxide dismutase (SOD) activity was quantified using the nitroblue tetrazolium reduction method [36], and CAT activity was determined through the potassium permanganate titration method [37]. Ascorbic acid (AsA) content was measured by the ferric chloride reduction method [38], and GSH content was assayed following the 2-nitrobenzenesulfonic acid reduction method [39]. Ascorbate peroxidase (APX) activity was determined using the H2O2 reduction method [33], and GR activity was measured with the GR kit (Catalog No. S0055) supplied by Biyuntian (Beyotime Biotechnology Co., Ltd., Shanghai, China). Additionally, the activities of DHAR and MDHAR were assayed according to the method proposed by Han [40]. Detailed procedures for the determination of all the aforementioned indicators are available in our previous study [33].
2.4. Extraction of Seeds RNA and cDNA Library Construction and Sequencing
Seed ribonucleic acid (RNA) was extracted by Huayueyang Rapid Universal Plant RNA Extraction Kit 3.0 (Huayueyang Biotechnology Co., Ltd., Beijing, China). The RNA concentration was measured by Qubit 4.0 fluorometer/MD enzyme-labeled (Thermo Fisher Scientific, Waltham, MA, USA), and RNA integrity detected by Qsep 400 bioanalyzer (Guangding Biotechnology Co., Ltd., Taiwan, China). Subsequently, the fragmentation buffer was added to break the RNA into short fragments, which were then used as templates for synthesizing the first-strand complementary deoxyribonucleic acid (cDNA) with six-base random hexamers. Then, buffer, dNTPs, and DNA polymerase were added to synthesize the second-strand cDNA, followed by purification of the double-stranded cDNA using DNA purification magnetic beads. The purified double-stranded cDNA underwent end repair, A-tail addition, and ligation with sequencing adapters. Fragment size selection was then performed using DNA purification magnetic beads, and PCR enrichment was carried out to obtain the final cDNA library. After library construction, its quality was tested, and upon meeting the required standards, the library was sequenced using the Illumina Novaseq 6000 (Illumina Co., Ltd., San Diego, CA, USA) platform.
To obtain clean data, raw sequencing data were processed through filtering to remove three types of reads, those containing adapters, those with an N proportion greater than 10%, and low-quality reads (reads in which bases with a quality score of Q ≤ 10 make up over 40% of the total bases in the total bases). The clean data was denovo assembled using the Trinity software (Version 2.13.2, Broad Institute and Hebrew University), and the redundant information in the transcripts were removed using the Corset software (Version 3.4, University of Melbourne, Australia), then non-redundant unigene was obtained [41]. These reads were then assembled into the species’ transcriptome sequences using Trinity. Subsequently, hierarchical clustering was performed, and the longest sequence in each cluster was selected as a unigene for downstream analysis, resulting in 127,103 unigenes (Table S1).
2.5. Differential Gene Screening
Following data filtering, differentially expressed genes (DEGs) were analyzed using DESeq2 software (Version 1.22.2, Heidelberg University, Germany). Subsequently, this analysis applied a correction method to adjust the p-values derived from hypothesis testing for multiple comparisons, generating the false discovery rate (FDR). DEGs were screened based on the following criteria: |log2 Fold Change| ≥ 1 and FDR < 0.05.
2.6. Functional Annotation of Differentially Expressed Genes, GO and KEGG Enrichment Analysis
Unigene sequences were aligned to the Kyoto Encyclopedia of Genes and Genomes (KEGG), Non-Redundant Protein Database (NR), Swiss-Prot Protein Sequence Database (Swiss-Prot), Gene Ontology (GO), Clusters of Orthologous Groups of Proteins/Eukaryotic Orthologous Groups (COG/KOG), and Translation of EMBL Nucleotide Sequence Database (TrEMBL) via DIAMOND BLASTX(Version 2.0.9, University of Tübingen, Baden-Württemberg, Germany) to predict their encoded amino acid sequences. Subsequently, the Hidden Markov Model (HMMER) was employed to query the protein families database (Pfam) for additional unigene annotation information. DEGs were functionally annotated using the GO database, while their involvement in specific biological pathways was inferred via the KEGG pathway annotation based on the results.
2.7. Weighted Gene Co-Expression Network Analysis
Genes with analogous expression patterns were clustered into several independent modules, and then explored the interrelationships between these modules and phenotypic characteristics. The expression matrix of genes was derived from the gene expression levels of the seeds with different water content before and after cryopreservation. Subsequently, the WGCNA package of R software (Version 1.6.6, University of Auckland, New Zealand) was used to establish a weighted gene co-expression network [42]. Key parameters for network construction were set as follows: soft threshold β = 14, fitting index R2 = 0.85, and average connectivity approached 0.
2.8. qRT-PCR Verification
Six key genes in the plant MAPK signaling pathway and the plant starch-sucrose metabolism signaling pathway, along with three key genes involved in oxidative stress, were identified. The mRNA sequences (coding sequences, CDS) of these genes were retrieved from PGDB. The primers for the target genes were designed by the online website IDT (http://sg.idtdna.com/Primerquest/Home/Index, accessed on: 14 October 2025, Table S2), and synthesized by Beijing Riboxingke Biotechnology Co., Ltd. The qRT-PCR was performed using the B532461-0001 miRNA Fluorogenic Quantitative PCR kit-dye method (Sangong bioengineering Co., Ltd., Shanghai, China), with GADPH as the internal reference gene, each sample included three biological replicates, and gene relative expression levels were calculated using the 2−ΔΔCt method.
2.9. Statistical Analysis
One-way analysis of variance (ANOVA) was performed using SPSS 17.0 (SPSS Inc., Chicago, IL, USA). Tables were constructed with Microsoft Excel 2013 (Microsoft Corp., Richmond, CA, USA). Figures were generated using Origin 2021 (OriginLab, Northampton, MA, USA) and R software (v1.6.6; University of Auckland, Auckland, New Zealand).
3. Results
3.1. Changes in Viability of Seeds
Based on the results of seed germination rates and the TTC staining, seeds with high-water content (21.56%) exhibited a significant decrease in viability after cryopreservation. In contrast, those with low-water content (4.35%) showed a marked increase in viability following the same treatment (Figure 1A,B, Supplementary Figures S1 and S2).
Figure 1.
Changes in viability and oxidative stress indexes in P. lactiflora seeds with different water content before and after cryopreservation. HW: seeds with high-water content, LW: seeds with low-water content, pre-LN: before liquid nitrogen preservation, post-LN: after liquid nitrogen preservation. (A) The seeds viability. (B) The germination rate of seeds. (C) O2·− content, (D) H2O2 content, (E)·OH content, (F) MDA content, (G) PCO content, (H) SOD content, (I) CAT content, (J) APX content, (K) GR content, (L) DHAR content, (M) MDHAR content, (N) AsA content, (O) GSH content. Different lowercase letters indicated that there was significant differences in seed before and after cryopreservation of the same water content gradient (p < 0.05).
3.2. Changes in Oxidative Stress Indicators of Seeds
After cryopreservation, the O2·−, H2O2 and ·OH content in seeds with high-water content (21.56%) significantly increased, while H2O2 and ·OH content significantly decreased and O2·− content significantly increased after cryopreservation for seeds with low-water content (Figure 1C–E). Seeds with high-water content (21.56%) showed significant increases in MDA and PCO content after cryopreservation, while seeds with low-water content (4.35%) showed significantly decreased MDA content, and the PCO content had no significant changes (Figure 1F,G).
After cryopreservation, the activities of SOD, APX, GR and the content of AsA in seeds with high-water content (21.56%) did not show significant changes, but for seeds with low-water content (4.35%), the activities of SOD, APX, and GR significantly increased, the content of AsA significantly decreased (Figure 1H,J,K,N). The CAT and DHAR activities of seeds with high-water content (21.56%) and low-water content (4.35%) both significantly increased after cryopreservation (Figure 1I,L). After cryopreservation, the content of GSH and the activity of MDHAR in the seeds with high-water content (21.56%) significantly increased, while the activity of MDHAR in seeds with low-water content (4.35%) did not show significant changes, and the content of GSH significantly decreased (Figure 1M,O).
3.3. Sequencing Data Analysis and Quality Assessment
The Illumina high-throughput sequencing platform was used to sequence 12 seed samples (before and after cryopreservation), yielding a total of 92.92 Gb of clean data. Each sample contributed at least 6 Gb of clean data, with the Q30 base percentage exceeding 93%. After filtering the raw sequencing data, high-quality reads were obtained.
Samples with high-water content before cryopreservation (HWC-Pre) and after cryopreservation (HWC-Post) clustered into one group, while those with low-water content before (LWC-Pre) and after (LWC-Post) cryopreservation formed another distinct group (Supplementary Figure S3). This clustering pattern indicated good intra-group repeatability, confirming that the samples were suitable for subsequent analyses.
Unigene sequences were aligned against KEGG, NR, Swiss-Prot, GO, COG/KOG, and Trembl via DIAMOND, after predicting their amino acid sequences, HMMER was used to align against Pfam for unigene annotations (Table S3).
3.4. Differentially Expressed Genes of Seeds
In total, 6936 DEGs were detected between before and after cryopreservation (Figure 2). Among them, 1224 genes were up-regulated and 1839 genes were down-regulated in high-water content seeds after cryopreservation. After cryopreservation, 2090 genes were up-regulated and 1783 genes were down-regulated in the seed with low-water content, but only 687 DEGs were common to both high- and low-water content seed after cryopreservation.
Figure 2.
Statistical charts of differentially expressed genes in P. lactiflora seeds with different water content before and after cryopreservation. (A) Volcano plot of differentially expressed genes in high-water content seeds. (B) Volcano plot of differentially expressed genes in low-water content seeds. (C) Statistical chart of the number of differentially expressed genes in seeds with different water contents. (D) Venn diagram of differentially expressed genes in seeds with different water contents.
3.5. GO Functional Enrichment Analysis of DEGs
The GO enrichment analysis of DEGs in high-water content seeds before and after cryopreservation, among the 50 GO terms with the lowest q-value, 30 functional subcategories were enriched in biological process, 2 functional subcategories enriched in cellular component, and 18 functional subcategories enriched in molecular function. While for the low-water content seed, 34 functional subcategories were enriched in the biological process category, and 16 functional subcategories in the molecular function category (Figure 3).
Figure 3.
GO functional enrichment analysis of differentially expressed genes before and after cryopreservation of P. lactiflora seeds with different water contents. (A) GO functional enrichment classification of differentially expressed genes of high-water content seeds. (B) GO functional enrichment classification of differentially expressed genes of low-water content seeds. (C) GO term enrichment analysis results of differentially expressed genes in high-water content seeds. (D) GO term enrichment analysis results of differentially expressed genes in low-water content seeds. The red font indicates the pathways that are collectively enriched in both comparison groups.
The items that were significantly enriched in both high- and low-water content seeds after cryopreservation were beta-glucosidase activity and glucosidase activity (Figure 3). Among them, in the terms of beta-glucosidase activity, 12 DEGs were significantly enriched in the seeds with high water content, five genes showed up-regulated expression and seven genes showed down-regulated expression. Seeds with low-water content showed significant enrichment of 13 DEGs, six genes showed up-regulated expression and seven genes showed downregulated expression. For glucosidase activity, the seeds with high-water content enriched 14 DEGs after cryopreservation, among which five genes were up-regulated and nine genes were down-regulated. However, the seeds with low-water content enriched 17 DEGs in glucosidase activity after cryopreservation, among which eight genes were up-regulated and nine genes were down-regulated. These items (beta-glucosidase activity and glucosidase activity) play an important role in the changes in viability of seeds with different water content after cryopreservation.
3.6. KEGG Metabolic Pathway Enrichment Analysis of DEGs
KEGG enrichment analysis of DEGs found that there were 771 DEGs enriched in 133 pathways in high-water content seeds, and 928 DEGs enriched in 132 pathways in low-water content seeds before and after cryopreservation. The most significantly enriched pathways of DEGs were mainly related to the biosynthesis of various plant secondary metabolites, the biosynthesis of secondary metabolites, the MAPK signaling pathway-plants, starch and sucrose metabolism pathways, and the synthesis of secondary metabolites such as isoflavones, hydroxy acids, and alkaloids (Figure 4). Among them, the genes showed significant differential expression after cryopreservation in the seeds with high- and low-water content were mainly enriched in the plant MAPK signaling pathway (ko04016) and the starch and sucrose metabolism pathway (ko00500).
Figure 4.
Scatter plot of KEGG enrichment results of differentially expressed genes before and after cryopreservation of P. lactiflora seeds with different water contents. (A) Scatter plot of KEGG enrichment results of seeds with high-water content. (B) Scatter plot of KEGG enrichment results of seeds with low-water content. The red font indicates the pathways that are collectively enriched in both comparison groups.
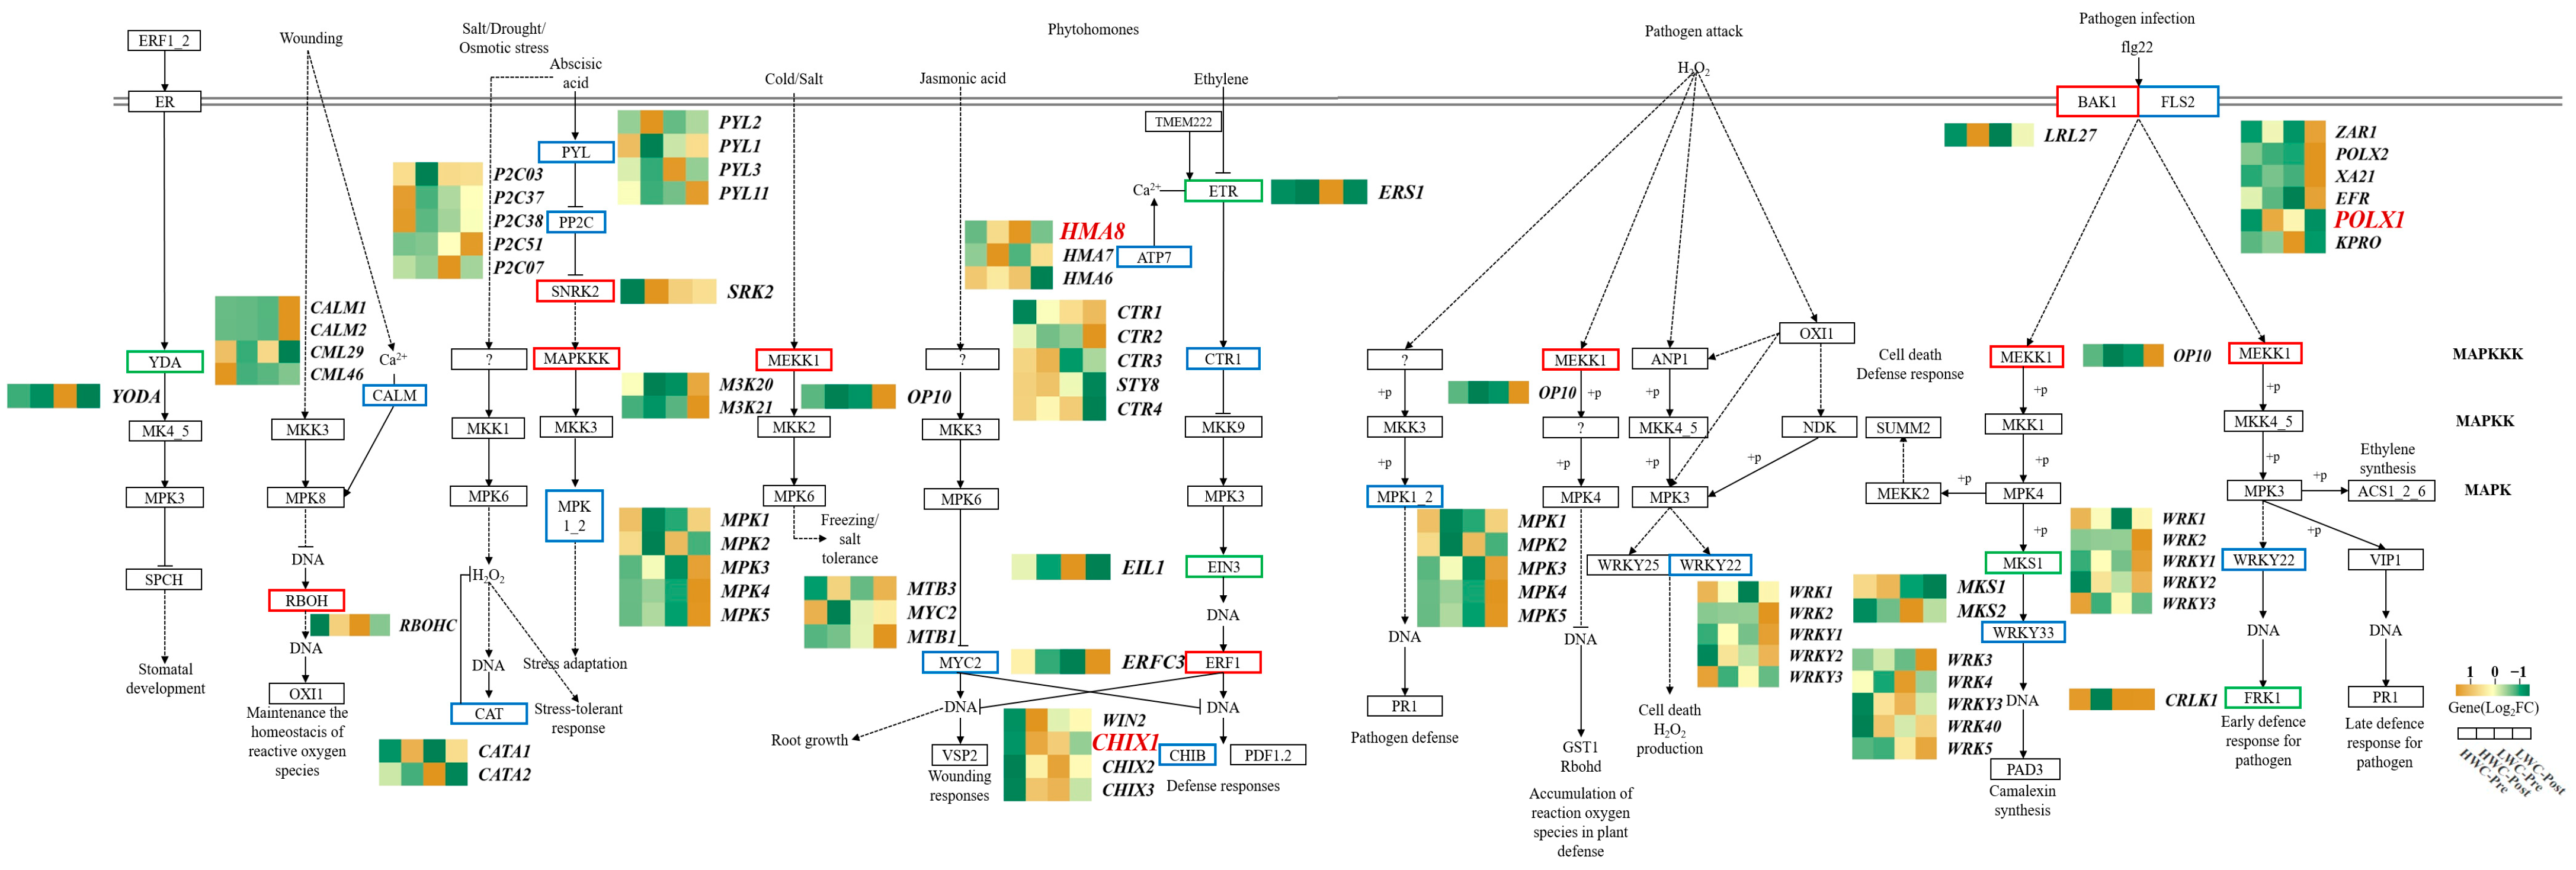
A total of 64 DEGs were involved in the MAPK signaling pathway–plant metabolic pathway before and after cryopreservation of seeds with high- and low-water content. Among them, the POLX1 of the receptor protein (FLS2), the HMA8 of the copper ion transport ATPase peptide (ATP7), and the CHIX1 of the alkaline endo-protease B (CHIB) showed up-regulated trend after cryopreservation of seeds with high-water content. However, for the seeds with low-water content, the expression trend showed a down-regulated, the expression trend was significantly negatively correlated with the change in seed viability, this indicated that POLX1, HMA8, and CHIX1 play important roles in the viability changes in seeds with different water content after cryopreservation (Figure 5).
- MAPK signaling pathway-plan
Figure 5.
MAPK signaling pathway. The enzymes marked in red are related to up-regulated genes, those marked in green are related to down-regulated genes, and those marked in blue are related to both up-regulated and down-regulated genes. The “?” serve as placeholders, indicating that the specific direct homologous genes at this node on this pathway have not yet been explicitly identified or labeled by the KEGG database.
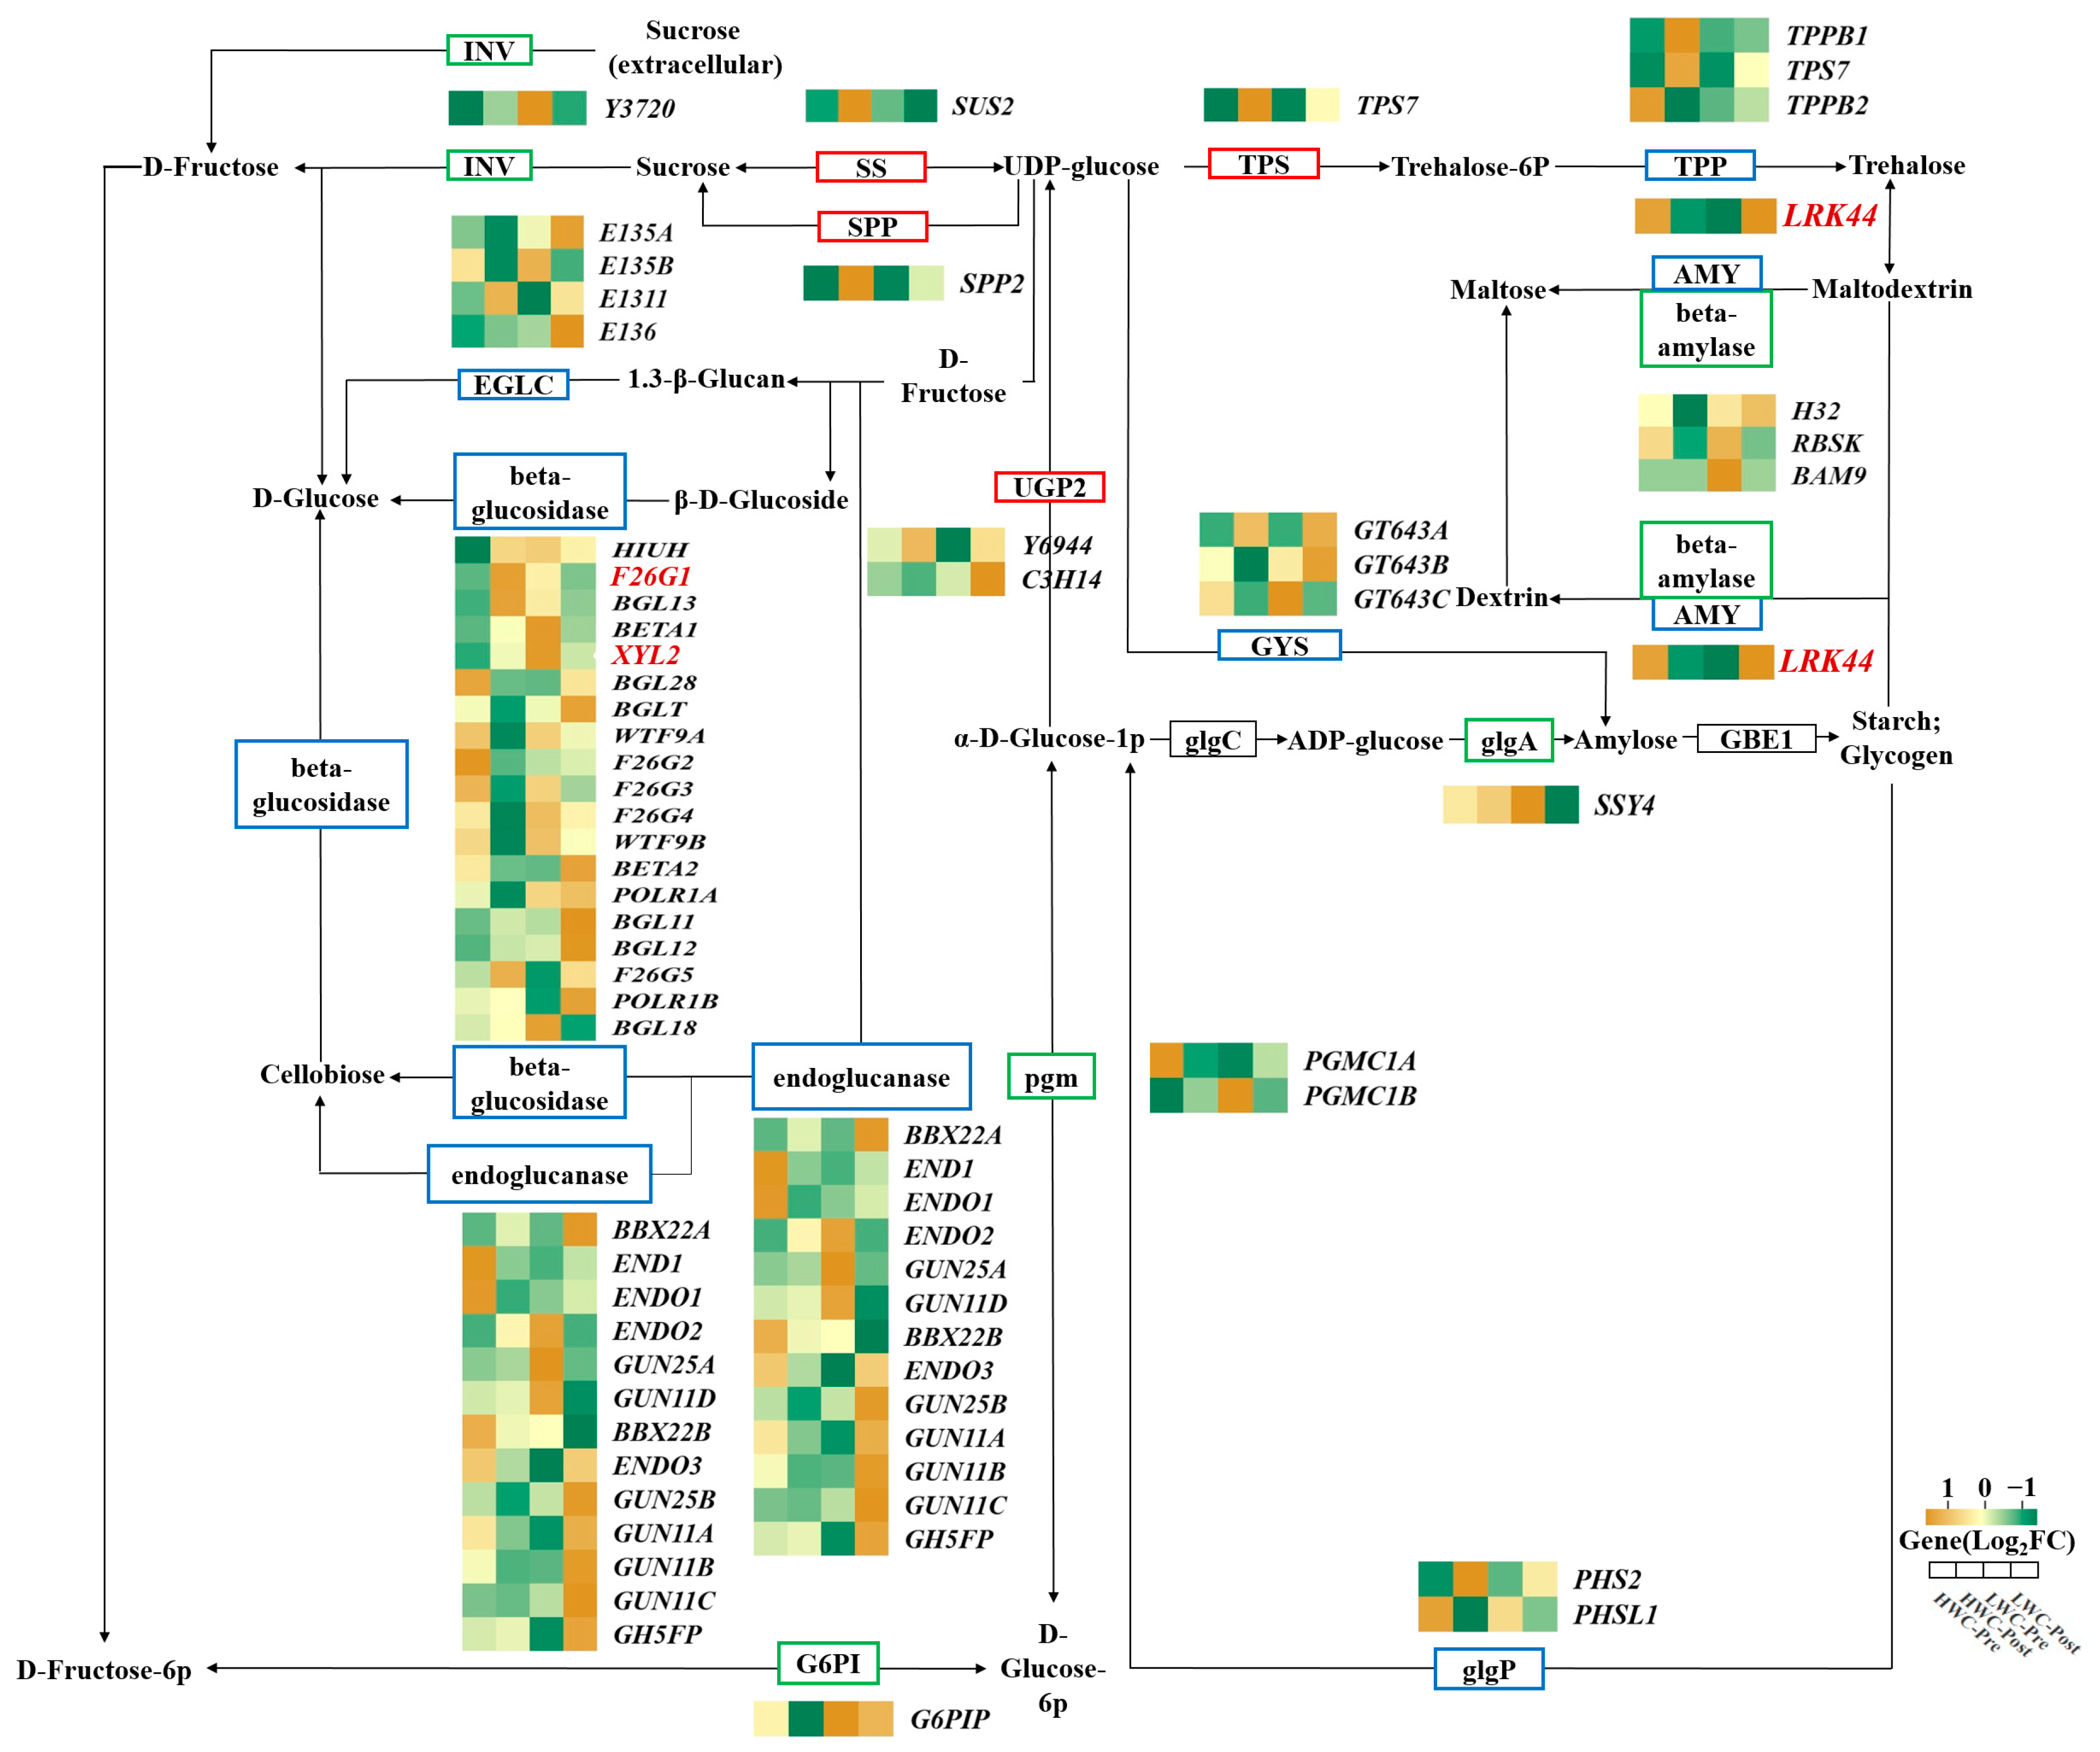
After cryopreservation, 34 DEGs were significantly enriched in the starch and sucrose metabolism pathway in the seeds with high-water content, and 31 DEGs in the seed with low-water content. Only six of these DEGs were co-enriched in both high- and low-water content seeds after cryopreservation (Figure 6). Among them, the LRK44 gene, which regulated the activity of amylase (AMY), showed a significant down-regulation in seeds with high-water content, and a significant up-regulation in seeds with low-water content, which was significantly positively correlated with the viability changes in the seeds. The F26G1 and XYL2 genes, which regulated the activity of beta-glucosidase, showed significant up-regulation in the seeds with high-water, and significant down-regulation in the seeds with low-water content. Their expression patterns were significantly negatively correlated with the viability changes in the two types of seeds. Therefore, in the starch and sucrose metabolism pathway, these three genes play a significant role in the changes in seed viability.
- Starch and sucrose metabolism
Figure 6.
Starch and sucrose metabolic signaling pathways. The enzymes marked in red are related to up-regulated genes, those marked in green are related to down-regulated genes, and those marked in blue are related to both up-regulated and down-regulated genes.
3.7. Weighted Gene Co-Expression Network Analysis
Genes with low expression were removed and the genes with stable expression in all seed samples, a total of 37,818 genes, were screened out. Based on the correlation of gene expression in seed samples, we constructed a gene clustering tree and divided modules, and merged the small modules with high similarity (module merging threshold was set at 0.25). A total of 27 modules were constructed (Figure 7A), the turquoise module contains the largest number of genes (6187), while the dark orange module contains the fewest genes (109), and the gray module includes 622 genes that are identified as ‘invalid genes’ as they showed low expression or stable expression across samples (Figure 7B,C).
Figure 7.
Weighted gene co-expression network analysis of P. lactiflora seeds with different water contents before and after cryopreservation. (A) Soft threshold selection schematic diagram, (B) module hierarchical clustering tree diagram, (C) correlation heatmap between modules and different samples, (D) correlation heatmap between modules.
To further explore the key factors causing viability changes in seeds with different water content after cryopreservation, a correlation analysis was conducted on the obtained modules and viability of seeds before and after cryopreservation. Among them, the gene expression pattern of the green module was negatively correlated with the viability change, while the gene expression pattern of the magenta module was positively correlated with the viability changes (Figure 7C). This indicated that the green and magenta modules play a crucial regulatory role in the viability changes after cryopreservation, these modules can be regarded as key modules.
Further analysis showed that there were 2504 genes in the green module and 1597 genes in the magenta module (Figure 7C). The most representative genes were selected within each module, which were referred to as the feature vector genes (ME), and then performed clustering processing on all the MEs of the modules. The higher the correlation between the modules, the stronger the correlation between the modules, and through the correlation analysis of ME, it was found that the correlation between the green module and the magenta module reached −0.86. Therefore, these two modules can be studied as modules related to the viability changes in seed, and the core genes can be identified from them (Figure 7C,D).
Through GO functional analysis, for the biological process category, both modules showed significant enrichment in cellular processes, metabolic processes, responses to stimuli, and biological regulation. Meanwhile, in the cellular component category, they were significantly enriched in cellular anatomical entities and protein-containing complexes. Additionally, regarding molecular function, both modules exhibited significant enrichment in binding and catalytic activity (Figure 8). Among them, these two key modules involved the pathways related to signal transduction, stress responses to external stimuli and stressors, and positive and negative regulation of biological processes.
Figure 8.
Co-expression network construction of the green and magenta module. (A) Expression profile of characteristic genes in the green module. (B) GO functional enrichment analysis of genes in the green module. (C) Expression profile of characteristic genes in the magenta module. (D) GO functional enrichment analysis of genes in the magenta module. (E) Grid diagram of the green module. (F) Grid diagram of the magenta module.
Furthermore, by constructing a gene co-expression network diagram, the core genes with high connectivity in the two modules were identified. The results showed that in the green module, five core genes were identified, WDL5, PMA4, FBL11, CHR28, and UXS2 (Figure 8E), and in the magenta module, five core genes, LEA34, METK5, DHN1, Y2608, and DECR2 (Figure 8F). Through the annotation of these genes, it was found that some of the core genes are related to cold stress response and oxidative stress, METK5 encodes the basic enzyme in the ethylene biosynthesis pathway, DECR2 is a key gene that regulates the activity of oxidoreductases, DHN1 (AT1G20440.1) is a cold stress-regulating gene (COR47).
3.8. Changes in Transcription Factors of Paeonia lactiflora Seeds
This study detected 3543 transcription factors belonging to 94 transcription factor families before and after cryopreservation of seeds with different water content. Among them, 48 transcription factor families in seeds with high-water content showed differential expression, totaling 118 transcription factors. While in seeds with low-water content, 50 transcription factor families showed differential expression, totaling 149 transcription factors. Based on the changes in the seeds with high- and low-water content, there were 12 transcription factors that were significantly related to the changes in seed viability (Supplementary Figure S4). Among them, LOB, NF-YB, B3, AP2/ERF-ERF1, AP2/ERF-ERF2, HSF, and SET were significantly positively correlated with the changes in seed viability, while C2H2, AUX/IAA, MYB-related1, MYB-related2, and RWP-RK were significantly negatively correlated.
3.9. qRT-PCR Verification of Differentially Expressed Genes
To verify the reliability of the transcriptome data, nine DEGs closely related to the viability changes in the seeds were selected. The qRT-PCR expression levels of these nine DEGs were highly consistent with the changes observed in RNA-Seq (Figure 9), which confirmed that the authenticity and reliability of the RNA-Seq results of this study.
Figure 9.
qRT-PCR verification of the nine DEGs. HWC-Pre: Seeds with high-water content before cryopreservation; HWC-Post: Seeds with high-water content after cryopreservation; LW C-Pre: Seeds with low-water content before cryopreservation; LWC-Post: Seeds with low-water content after cryopreservation. Different lowercase letters indicated that there were significant differences in seeds before and after cryopreservation of the same water content gradient (p < 0.05).
4. Discussion
Cryopreservation serves as an ideal method for the long-term storage of plant germplasm resources, while water content is one of the key factors influencing its storage effectiveness [6]. In this study, at a relatively high-water content of 21.56%, seeds exhibited significantly reduced viability after cryopreservation. Concomitantly, there was abnormal accumulation of ROS, along with membrane lipid and protein damage induced by this ROS accumulation (Figure 1). In contrast, when seed water content was reduced to 4.35%, cryopreserved seeds showed a significant increase in viability; meanwhile, the lower water content had a certain alleviating effect on ROS accumulation and the oxidative stress triggered by ROS after cryopreservation (Figure 1). Similarly, this phenomenon was also observed in the cryopreservation of P. emodi seeds, when the seed water content was relatively high (18.33%), the viability of the seeds significantly decreased after cryopreservation, but when the seed water content dropped to 7.07%, the seeds viability increased, and the changes in the ROS were also observed [32]. This phenomenon may be caused by the excessive water content of the seeds, which during the freeze–thaw process of cryopreservation, cells will form ice crystals, which will damage the cell membranes and reduce the cell viability [43]. These results substantiate that water content is one of the most important factors affecting the viability changes in Chinese herbaceous peony (P. lactiflora) seeds after cryopreservation, and the oxidative stress induced by ROS is one of the main reasons for the differences in the viability changes.
Notably, although seeds with low-water content exhibited increased viability after cryopreservation, their viability remained significantly lower than that of non-cryopreserved seeds with high-water content (Figure 1). This finding is consistent with Chmielarz’s research on cryopreservation of cherry (Cerasus avium) seeds, while cryopreservation enhanced the viability of low-water content seeds, but the magnitude of this increase was considerably lower than that of freshly harvested seeds with natural water content without cryopreservation [44]. This was attributed to seed water content below 10%, where the cytoplasm within the dehydrated cells undergo vitrification, forming a glass-like state, similar to a solid while retaining the physical properties of a liquid [45]. While the glassy-like cytoplasmic state reduces damage to cell membranes and other cellular components during cryopreservation, the cold stress imposed by cryopreservation can also stimulate cells [46], thereby enhancing post-cryopreservation seed viability. However, excessive dehydration deprives seeds of the water required for germination. Consequently, seeds with low-water content exhibit markedly reduced viability before cryopreservation. Collectively, these results indicate that a lower water content does not equate to better outcomes in seed cryopreservation of seeds. Only when the water content of the seeds falls within a narrowly appropriate range can seeds maintain their viability for the longest time.
With the development of molecular biology, transcriptomics has become a useful means for studying the mechanisms underlying changes in seed viability [47,48]. In this study, utilized transcriptome sequencing technology identified 6249 DEGs in the high (21.56%) and low-water content (4.35%) Chinese herbaceous peony (P. lactiflora) seeds before and after cryopreservation. Among them, 1224 up-regulated genes and 1839 down-regulated genes were observed in the high-water content seeds after cryopreservation, 2090 up-regulated genes and 1783 down-regulated genes were found in the low-water content seeds after cryopreservation, and the GO enrichment analysis of the DEGs showed that the main common enriched items before and after cryopreservation of the two types of seeds were all related to metabolic processes (Figure 2 and Figure 3). This might be due to reducing the respiratory metabolic rate of the biological material, resulting in alleviating the decline in viability [2,3]. Secondly, one of the primary mechanisms by which plant cells respond to external stimuli is through metabolite regulation, which involves metabolism or the generation of secondary metabolites to adapt to the biological changes induce by cryopreservation [49]. In addition, the KEGG metabolic pathway analysis revealed that after cryopreservation of the seeds with different water content in this study, a large number DEGs were significantly enriched in the ‘MAPK signaling pathway- plant’ and ‘starch- sucrose metabolism’ pathways (Figure 4). Previous studies have shown that the MAPK signaling pathway is widely present in plants and actively participates in various signal transmission processes, which amplifies and transmits non-biological stress signals step by step through phosphorylation, and is the most common and fundamental regulatory method in the biological system, as well as one of the important mechanisms for plant stress responses [50]. Similarly, starch-sucrose metabolism also plays a significant role in plant stress responses, especially under low-temperature stress conditions [51]. The above findings indicated that the viability changes seen in this study may mainly involve in the regulation of the ‘MAPK signaling pathway- plant’ and the ‘starch- sucrose metabolism’ pathways.
Studies have shown that the members of the mitogen-activated protein kinase MAPK, MAPKK, and MAPKKK families play crucial roles in the signal transduction pathways of plants in response to cold stress. When plants are exposed to cold stress, the concentration of Ca2+ ions in the cells will increase, activating the MAPK cascade reaction, this reaction sequentially phosphorylates through MAPKKK to MAPKK and then to MAPK, transferring the cold signal step by step to downstream transcription factors and protein kinases and other targets, completing the transmission process of the cold signal [52,53]. Existing studies have also show that the downstream of the plant’s cold response mechanism mainly relies on the ICE-CBF (DREB)-COR signaling pathway, ICE1 (inducer of CBF expression) binds to the promoter regions of CBF (C-repeat-binding factor) genes to activate their expression, then regulates the plant’s adaptability to low temperatures [54]. Among them, CBF is a transcription factor of the AP2/ERF family, while COR (cold-regulated gene) is a gene that is activated only under low temperature conditions, and is responsible for generating proteins that regulate low temperatures. The CORs regulated by CBF have at dozens of types (COR47, COR27, COR78, etc.), and their encoded proteins are synthesized under low temperatures and stabilize the structure of cells and proteins, restore the balance of substances within the plant, and enhance the plant’s adaptability to low temperatures. The CBF transcription factor is regarded as upstream of cold stress [55]. In this study, the MAPK signal transduction pathway was activated in the Chinese herbaceous peony (P. lactiflora) seeds, thereby mediating the differential expression of downstream ICE-CBF (DREB)-COR signaling pathway genes. Among them, for seeds with low-water content, the expressions of DRE1D and DRE2A were significantly up-regulated after cryopreservation, while COR27 was significantly up-regulated and the expression of DRE2 was significantly down-regulated. While for the seeds with high-water content, the expression of DRE2 was significantly down-regulated after cryopreservation. In addition, DHN1, one of the core genes of the magenta module in the WGCNA analysis, it was significantly down-regulated during the cryopreservation of seeds with high-water content, and significantly up-regulated in the seeds with low-water content (Figure 5, Figure 7, and Figure 8). Previous studies have shown the homologous gene of DHN1 in arabidopsis (A. thaliana) (AT1G20440.1) is the cold-regulating gene COR47, plants overexpressing COR47 have ultra-low temperature tolerance [56]. When plants are subjected to low temperatures, the ICE-CBF-COR signaling pathway is activated, promoting the expression of COR genes, which enhances the plant’s adaptability to low temperatures [57,58]. Therefore, these results indicated that in the cryopreservation of different water content Chinese herbaceous peony (P. lactiflora) seeds, the MAPK signal transduction pathway is activated, mediating the differential expression of downstream ICE-CBF (DREB)-COR signaling pathway genes, then participating in the mechanism of the difference in seed viability after cryopreservation.
Studies also show that hormones play a crucial role in the MAPK signaling pathway and actively participate in the regulation of the cold response mechanism [59]. Under low-temperature conditions, abscisic acid (ABA), jasmonic acid (JA), and ethylene in plants increase rapidly, these hormones improve cold tolerance in plants by activating the antioxidant system and inducing the up-regulation of genes related to cold responses [60]. Under low-temperature conditions, plants accumulate a large amount of ABA, which binds to its receptor protein PYL (abscisic acid receptor), then inhibiting the dephosphorylation activity of PP2C (protein phosphatase 2C gene), phosphorylating protein kinase SnRK2 (serine/threonine-protein kinase), and phosphorylating downstream transcription factors ABF, activating the expression of genes containing ABRE elements in the promoter region, plants respond to low temperatures through mechanisms such as regulating dormancy [61,62]. In the ABA signaling pathway of this study, the three key components- PYL, PP2C, and SnRK2 were all affected by cryopreservation. They exhibited significant changes in their transcriptional levels, including both up-regulation and down-regulation, which subsequently encoded corresponding proteins to participate in the ABA signaling process and enhance plant tolerance to ultra-low temperature. This corresponds with existing findings, such as the study on the effects of low temperature on the genomic expression of passion flower (Passiflora edulis), where both up-regulation and down-regulation of PP2C and SnRK2 genes were observed in the ABA signaling pathway [63]. Meanwhile, JA also can enhance plant cold tolerance and interact with the ABA pathway, MYC2 being the core transcription factor in the jasmonic acid signaling pathway [64]. In this study, the key genes of the jasmonic acid pathway, MYC2 family members, exhibited both up-regulated and down-regulated expression, indicating that this pathway plays a significant role in Chinese herbaceous peony (P. lactiflora) seed response to cryopreservation (Figure 5). In addition, the ethylene-mediated MAPK signaling pathway plays a crucial role in plant low-temperature response [65]. In this study, the MAPK pathway was enriched with a large number DEGs, among which HMA8 at ATP7 and CHIX1 at CHIB were significantly up-regulated after cryopreservation of high-water content seeds, but significantly down-regulated for low-water content seeds, a trend that showed a significant negative correlation with seed viability changes before and after cryopreservation (Figure 5). In summary, the MAPK signaling pathway involved in the cryopreservation of Chinese herbaceous peony (P. lactiflora) seeds with different water content mediates the roles of ABA, JA, and ethylene, playing a crucial role in the viability changes in the seeds after cryopreservation.
Starch-sucrose metabolism also plays an important role in plant low-temperature stress; studies showed that starch is a key molecule that regulates plants’ responses to extreme temperature stimuli [51]. Under low-temperature treatment, plants can mobilize their starch reserves to provide energy and carbon, then released sugars and other derivative metabolites, to maintain the growth and development of plants at low temperatures [66]. Based on the KEGG analysis, it was found that there are two main metabolic pathways for starch synthesis, one of which involves the conversion of α-D-glucose-1-phosphate to UDP-glucose under the catalysis of UTP-glucose-1-phosphate uridylyltransferase (UGP2), followed by the joint action of glycogen synthase (GYS) and granule-bound starch synthase (WAXY) to produce amylose, which is then converted to starch under the catalysis of 1,4-α-glucan branching enzyme (GBE1). Another metabolic pathway involves the conversion of α-D-glucose-1-phosphate to ADP-glucose under the catalysis of glucose-1-phosphate adenylyltransferase (glg C). This is followed by the formation of amylose through the joint catalysis of starch synthase (glg A) and WAXY, and finally the production of starch under the action of GBE1. Among them, UGP2 functions in the early stages of the metabolic pathway, using D-glucose-1-phosphate as a substrate to catalyze the formation of UDP-glucose, and the expression of UGP2 affects its activity and UDP-glucose production, then influencing starch synthesis [67]. In this study, the expression of UGP2 in seeds with low-water content was significantly up-regulated after cryopreservation, while there was no significant difference in the expression of seeds with high-water content (Figure 6). It appears that the early starch metabolism reaction circuit catalyzed by UGP2 was not involved in the viability changes in the seeds after cryopreservation.
However, in the starch-sucrose metabolic pathway, besides UGP2, starch synthase (glg A) also plays a crucial role, where ADP-glucose is catalyzed by glg A to produce amylose during seed starch and sucrose metabolism, and amylose is then converted into starch under the catalysis of 1,4-α-glucan branching enzyme (GBE1). In this study, the expression of glgA in seeds with low-water content was significantly down-regulated after cryopreservation (Figure 6). While the process in which the starch is catalyzed into maltodextrin, dextrin, and maltose is an important stage for plants to respond to low-temperature stress by increasing energy supply [68]. Among them, amylase (AMY) played a significant role as an important catalyst and during the cryopreservation of seeds, the AMY regulatory gene LRK44 was significantly down-regulated after cryopreservation of seeds with high-water content and significantly up-regulated for seeds with low-water content (Figure 6). These results indicated that during cryopreservation starch is converted into sugars under the action of AMY, thereby participating in the changes in seed viability, but the specific mechanism of action is worthy of our further in-depth exploration.
In addition, sucrose can act as a cryoprotectant, ROS scavenger, and signaling molecules to protect the cell membrane structure and prevent cells from stress damage [69]. Among them, sucrose synthase (SS) has the functions of decomposing and synthesizing sucrose and is a key enzyme in plant sucrose metabolism [70]. In the seed starch and sucrose metabolism pathway, sucrose is decomposed by sucrose synthase to produce UDP-glucose and D-Fructose, while UDP-glucose is synthesized by sucrose synthase to produce sucrose [71]. In this study, seeds with high-water content showed a significant up-regulation of sucrose synthase expression after cryopreservation (Figure 6), indicating that the seeds respond to external stimuli by accelerating sucrose synthesis and degradation, which consistent with the earlier findings [72,73], demonstrating that sucrose synthase plays a crucial role in plant cold stress response regulation. Moreover, a higher sucrose content can maintain the stability of the seed cell membrane, reducing the damage to membrane lipids [74]. In this study, UDP-glucose was synthesized into sucrose under the catalysis of sucrose synthase and sucrose 6-phosphatase (SPP), then SUS2 at sucrose synthase and SPP2 at sucrose 6-phosphatase (SPP) were significantly up-regulated in seeds with either water content, while Y3720 at β-fructofuranidase (INV), a key enzyme in the sucrose decomposition pathway, was significantly down-regulated in the seed with low-water content (Figure 6). This indicates that seeds with low-water content can maintain a higher sucrose content compared to those with high-water content. Similarly, from a physiological perspective, the membrane lipid damage index MDA of the seeds with different water content showed that the seeds with high-water content suffered more severe membrane lipid damage, and we speculated that this might be related to the lower sucrose content inside the seeds. And beta-glucosidase is a hydrolase that serves as the rate-limiting enzyme in cellulose degradation, primarily catalyzing the conversion of cellodextrin to cellobiose during seed starch and sucrose metabolism, with cellobiose further being converted to glucose under the catalysis of beta-glucosidase, and it can also catalyze the production of glucose from β-D-glucoside [75]. In this study, the genes F26G1 and XYL2 at β-glucosidase were significantly up-regulated in the seed with high-water content and significantly down-regulated in the seed with low-water content (Figure 6). This indicated that these genes served a key role in the changes in seed viability following cryopreservation. These findings indicated that, in the starch and sucrose metabolism pathways, starch synthase (glg A) regulates starch synthesis, amylase (AMY) controls the conversion of starch to sugars, beta-glucosidase modulates glucose synthesis, and sucrose synthase governs the breakdown and synthesis of sucrose, which are key regulatory steps in the viability changes in seeds with different water content after cryopreservation. The role of beta-glucosidase was particularly prominent, and the genes involved are key regulatory genes that require further in-depth study.
Transcription factors function critically in the development of plant seeds and variations in seed vigor [76], and study of their structure and function is an important task in fields such as plant molecular biology. In this study, transcription factors played a significant role in the viability changes in seeds after cryopreservation. LOB, NF-YB, B3, AP2/ERF-ERF1, AP2/ERF-ERF2, HSF, and SET positively regulated the viability changes in seeds after cryopreservation, while C2H2, AUX/IAA, MYB-related1, MYB-related2, and RWP-RK negatively regulated these changes (Figure S4). Among them, AP2/ERF, WRKY, NAC, C2H2, MYB, and bHLH were confirmed to actively participate in plant cold stress responses [77,78,79]. This is similar to the ICE-CBF(DREB)-COR signaling pathway as the most extensively studied low-temperature response pathway, with its core node CBF, a member of the AP2/ERF family, playing a crucial role in plant cold stress. In this study, the expressions of AP2/ERF-ERF and AP2/ERF-ERF were significantly positively correlated with the viability changes in seeds with different water content after cryopreservation. The C2H2 zinc finger protein is co-expressed in parallel with the CBF gene to induce the expression of COR genes, and suppression of its expression in arabidopsis (A. thaliana) significantly reduced the plant’s cold tolerance [80,81]. However, in this study the low expression of C2H2 improved the viability of low-water content seeds after cryopreservation, though the specific reasons require further analysis (Figure S4). In addition, the MYB family is the most common and functionally robust class of transcription factors in plants, playing a key role in plant low-temperature response [82]. In this study, the expression of MYB-related1 and MYB-related2 showed a significant negative correlation with the viability changes in seeds with different water content after cryopreservation, indicating their involvement in the stress response during cryopreservation of seeds with varying water content. Thus, these transcription factors can be used for the study of the mechanisms of the differences in plant cell viability after cryopreservation.
5. Conclusions
This study investigated the mechanism underlying seed viability changes after cryopreservation, focusing on the impact of water content variations, using physiological and transcriptomic data. The results demonstrated that seeds with high-water content (21.56%) exhibited a significant decline in viability after cryopreservation. Concurrent with this viability decline were the abnormal accumulation of reactive oxygen species (ROS) and subsequent ROS-induced membrane lipid damage. In contrast, seeds with low-water content (4.35%) showed enhanced viability after cryopreservation. For these low-water content seeds, a range of antioxidant substances were activated, leading to significantly reduced ROS levels and consequent oxidative damage. Notably, differential expression of genes in plant MAPK signaling pathway and starch-sucrose metabolism pathway was identified as a critical factor contributing to these viability differences. Furthermore, weighted gene co-expression network analysis concluded that two core genes regulating viability changes in seeds with different water content after cryopreservation. These included DHN1, a key component of the ICE-CBF (DREB)-COR plant cold stress response pathway, and LEA34, which serves as a crucial role in scavenging ROS and suppressing membrane lipid peroxidation. This study has pinpointed a series of potential target genes associated with viability changes in seeds with different water content after cryopreservation, providing a broader perspective for in-depth exploration of the molecular regulatory mechanisms governing cell viability changes after cryopreservation.
Supplementary Materials
The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/horticulturae11121494/s1, Figure S1: Germination of seeds under different preservation methods; Figure S2: TTC staining of seeds under different preservation methods; Figure S3: Principal component analysis (PCA) of the gene expression profiles of high and low water content seeds before and after cryopreservation; Figure S4: Analysis of the expression profiles of transcription factors (TFs) regulating the viability of P. lactiflora seeds with different water content before and after cryopreservation; Table S1: The quality analysis of sequencing data; Table S2: qRT-PCR primer information table; Table S3: Transcriptome data in the seven databases and success rate statistics of the gene annotation.
Author Contributions
R.R. designed the research, conceived the project, supervised the analysis, drafted and critically Revised the manuscript. Z.J. completed the experiment, analyzed the data and drafted the manuscript. Q.Z. and B.Z. provided assistance during the experiment. X.Y. provided support on the experiment equipment. All authors have read and agreed to the published version of the manuscript.
Funding
This research was supported by the National Natural Science Foundation (No. 32201613, 32572128). Youth Scientific Research Project of Shanxi Basic Research Program (No. 202103021223170). Shanxi postdoctoral special grant fund (No. 6K245520001752).
Institutional Review Board Statement
The authors declare that all the experimental research studies on plants, including the collection of plant material, were carried out in accordance with relevant institutional, national, and international guidelines and legislation.
Informed Consent Statement
Not applicable.
Data Availability Statement
All data generated or analyzed in the course of this study are available in ‘Supplementary Materials’ and the ‘Sequence Reading Archive (https://ngdc.cncb.ac.cn/gsa/browse/CRA029089, accessed on 14 October 2025)’ under accession numbers CRA029089.
Acknowledgments
We particularly thank Barbara M. Reed for editing the manuscript. We are grateful to Liujun Shi for their assistance in the material collection.
Conflicts of Interest
The authors declare that they have no conflict of interest.
References
- Pritchard, H.W. Cryopreservation of seeds. Methods Mol. Biol. 1995, 38, 133–144. [Google Scholar] [PubMed]
- Harding, K. Genetic integrity of cryopreserved plant cells: A review. Cryoletters 2004, 25, 3–22. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, J.W.; Ozudogru, E.A.; Li, J.; Wang, M.R.; Bi, W.L.; Lambardi, M.; Wang, Q.C. Cryobiotechnology of forest trees: Recent advances and future prospects. Biodivers. Conserv. 2018, 27, 795–814. [Google Scholar] [CrossRef] [Scilit]
- Benson, E.E. Cryopreservation of phytodiversity: A critical appraisal of theory & practice. Crit. Rev. Plant Sci. 2008, 27, 141–219. [Google Scholar] [CrossRef] [Scilit]
- Panis, B.; Lambard, M. Status of cryopreservation technologies in plants (crops and forest trees). In Proceedings of the The Role of Biotechnology, Turin, Italy, 5–7 March 2005; pp. 43–54. [Google Scholar]
- Chmielarz, P. Cryopreservation of dormant European ash (Fraxinus excelsior) orthodox seeds. Tree Physiol. 2009, 29, 1279–1285. [Google Scholar] [CrossRef] [Scilit]
- Leopold, A.C.; Sun, W.Q.; Bernal-Lugo, I. The glassy state in seeds: Analysis and function. Seed Sci. Res. 1994, 4, 267–274. [Google Scholar] [CrossRef] [Scilit]
- Generoso, A.L.; Carvalho, V.S.; Walter, R.; Campbell, G.; Araújo, L.S.; Santana, J.G.S.; Cunha, M. Mature-embryo culture in the cryopreservation of passion fruit (Passiflora edulis Sims) seeds. Sci. Hortic. 2019, 256, 108638. [Google Scholar] [CrossRef] [Scilit]
- Chen, G.Q.; Ren, L.; Zhang, J.; Reed, B.M.; Shen, X.H. Cryopreservation affects ROS-induced oxidative stress and antioxidant response in Arabidopsis seedlings. Cryobiology 2015, 70, 38–47. [Google Scholar] [CrossRef] [Scilit]
- Huang, B.; Zhang, J.M.; Chen, X.L.; Xin, X.; Zhou, Y.C. Oxidative damage and antioxidative indicators in 48 h germinated rice embryos during the vitrification-cryopreservation procedure. Plant Cell Rep. 2018, 37, 1325–1342. [Google Scholar] [CrossRef] [Scilit]
- Ren, R.; Li, Z.; Zhang, L.; Zhou, H.; Jiang, X.; Liu, Y. Enzymatic and nonenzymatic antioxidant systems impact the viability of cryopreserved Paeonia suffruticosa pollen. Plant Cell Tiss. Org. 2021, 144, 233–246. [Google Scholar] [CrossRef] [Scilit]
- Dalle-Donne, I.; Rossi, R.; Giustarini, D.; Milzani, A.; Colombo, R. Protein carbonyl groups as biomarkers of oxidative stress. Clin. Chim. Acta 2003, 32, 23–38. [Google Scholar] [CrossRef] [Scilit]
- Halliwell, B. Reactive species and antioxidants. Redox biology Is a fundamental theme of aerobic life. Plant Physiol. 2006, 141, 312–322. [Google Scholar] [CrossRef] [Scilit]
- Rattanawong, K.; Koiso, N.; Toda, E.; Kinoshita, A.; Tanaka, M.; Tsuji, H.; Okamoto, T. Regulatory functions of ROS dynamics via glutathione metabolism and glutathione peroxidase activity in developing rice zygote. Plant J. 2021, 108, 1097–1115. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Terai, Y.; Ueno, H.; Ogawa, T.; Sawa, Y.; Miyagi, A.; Kawai-Yamada, M.; Ishikawa, T.; Maruta, T. Dehydroascorbate reductases and glutathione set a threshold for high-light-induced ascorbate accumulation. Plant Physiol. 2020, 183, 112–122. [Google Scholar] [CrossRef] [Scilit]
- Zhang, T.; Ma, M.; Chen, T.; Zhang, L.; Fan, L.; Zhang, W.; Wei, B.; Li, S.; Xuan, W.; Noctor, G. Glutathione-dependent denitrosation of GSNOR1 promotes oxidative signalling downstream of H2O2. Plant Cell Environ. 2020, 43, 1175–1191. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Uchendu, E.E.; Leonard, S.W.; Traber, M.G.; Reed, B.M. Vitamins C and E improve regrowth and reduce lipid peroxidation of blackberry shoot tips following cryopreservation. Plant Cell Rep. 2010, 29, 25–35. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Uchendu, E.E.; Muminova, M.; Gupta, S.; Reed, B.M. Antioxidant and anti-stress compounds improve regrowth of cryopreserved Rubus shoot tips. In Vitr. Cell. Dev. Biol.—Plant. 2010, 46, 386–393. [Google Scholar] [CrossRef] [Scilit]
- Jia, M.X.; Jiang, X.R.; Xu, J.; Di, W.; Shi, Y.; Liu, Y. CAT and MDH improve the germination and alleviate the oxidative stress of cryopreserved Paeonia and Magnolia pollen. Acta Physiol. Plant. 2018, 40, 37–47. [Google Scholar] [CrossRef] [Scilit]
- Gupta, A.S.; Heinen, J.L.; Holaday, A.S.; Burke, J.J.; Allen, R.D. Increased resistance to oxidative stress in transgenic plants that overexpress chloroplastic Cu/Zn superoxide dismutase. Proc. Natl. Acad. Sci. USA 1993, 90, 1629–1633. [Google Scholar] [CrossRef] [Scilit]
- Fang, J.Y.; Wetten, A.; Johnston, J. Headspace volatile markers for sensitivity of cocoa (Theobroma cacao L.) somatic embryos to cryopreservation. Plant Cell Rep. 2008, 27, 453–461. [Google Scholar] [CrossRef] [Scilit]
- Zhang, D.; Ren, L.; Chen, G.; Zhang, J.; Reed, B.; Shen, X. ROS-induced oxidative stress and apoptosis-like event directly affect the cell viability of cryopreserved embryogenic callus in Agapanthus praecox. Plant Cell Rep. 2015, 34, 1499–1513. [Google Scholar] [CrossRef] [Scilit]
- Jia, M.X.; Shi, Y.; Di, W.; Jiang, X.R.; Xu, J.; Liu, Y. ROS-induced oxidative stress is closely related to pollen deterioration following cryopreservation. In Vitr. Cell. Dev. Biol.—Plant 2017, 53, 433–439. [Google Scholar] [CrossRef] [Scilit]
- Mostek, A.; Dietrich, M.A.; Słowińska, M.; Ciereszko, A. Cryopreservation of bull semen is associated with carbonylation of sperm proteins. Theriogenology 2017, 92, 95–102. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Shaliutina-Kolešová, A.; Cosson, J.; Lebeda, I.; Gazo, L.; Shaliutina, O.; Dzyuba, B.; Linhart, O. The influence of cryoprotectants on sturgeon (Acipenser ruthenus) sperm quality, DNA integrity, antioxidant responses, and resistance to oxidative stress. Anim. Reprod. sci. 2015, 159, 66–76. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, X.; Li, N.; Li, W.; Gao, X.; Liu, L. Advances in transcriptomics in the response to stress in plants. Gllob. Med. Genet. 2020, 7, 30–34. [Google Scholar] [CrossRef] [Scilit]
- Hu, J.; Zhu, T.; Ling, J.; Yao, C.; Lu, N.; Kong, L.; Zhang, H.; Wang, J. Integrated transcriptome and physiological analysis reveal the molecular mechanism of the osmotic-responses induced by cryoprotectants in Norway spruce embryogenic tissue. Ind. Crop. Prod. 2023, 195, 116440. [Google Scholar] [CrossRef] [Scilit]
- Htwe, C.S.S.; Rajkumar, S.; Pathania, P.; Agrawal, A. Transcriptome profiling during sequential stages of cryopreservation in banana (Musa AAA cv Borjahaji) shoot meristem. Plants 2023, 12, 1165. [Google Scholar] [CrossRef] [Scilit]
- Ren, L.; Zhang, D.; Chen, G.; Reed, B.; Shen, X.; Chen, H. Transcriptomic profiling revealed the regulatory mechanism of arabidopsis seedlings response to oxidative stress from cryopreservation. Plant Cell Rep. 2015, 34, 2161–2178. [Google Scholar] [CrossRef] [Scilit]
- Wan, Y.; Zhang, M.; Hong, A.; Lan, X.; Yang, H.; Liu, Y. Transcriptome and weighted correlation network analyses provide insights into inflorescence stem straightness in Paeonia lactiflora. Plant Mol. Biol. 2020, 102, 239–252. [Google Scholar] [CrossRef] [Scilit]
- Xu, S.Y.; Liu, W.L.; Liu, X.B.; Qin, C.; He, L.Q.; Wang, P.P.; Kong, L.Y.; Chen, X.; Liu, Z.Y.; Ma, W. DUS evaluation of nine intersubgeneric hybrids of Paeonia lactiflora and fingerprint analysis of the chemical components in the roots. Front. Chem. 2023, 11, 1158727. [Google Scholar] [CrossRef] [Scilit]
- Ren, R.; Zhou, H.; Zhang, L.; Jiang, X.; Zhang, M.; Liu, Y. ROS-induced PCD affects the viability of seeds with different moisture content after cryopreservation. Plant Cell Tiss. Org. 2022, 148, 623–633. [Google Scholar] [CrossRef] [Scilit]
- Ji, Z.; Guo, J.; Huang, J.; Zhu, Q.; Ren, R. Effects of oxidative stress on the changes of viability of Paeonia lactiflora seeds with different water content before and after cryopreservation. Cryobiology 2024, 117, 105165. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Khan, M.; Hu, J.; Dahro, B.; Ming, R.; Zhang, Y.; Wang, Y.; Alhag, A.; Li, C.; Liu, J. ERF108 from Poncirus trifoliata (L.) Raf. functions in cold tolerance by modulating raffinose synthesis through transcriptional regulation of PtrRafS. Plant J. 2021, 108, 705–724. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gogorcena, Y.; Iturbe-Ormaetxe, I.; Escuredo, P.R.; Becana, M. Antioxidant defenses against activated oxygen in pea nodules subjected to water stress. Plant Physiol. 1995, 108, 753–759. [Google Scholar] [CrossRef] [Scilit]
- Walters, C.; Wheeler, L.; Stanwood, P.C. Longevity of cryogenically stored seeds. Cryobiology 2004, 48, 229–244. [Google Scholar] [CrossRef]
- Prochazkova, D.; Sairam, R.K.; Srivastava, G.C.; Singh, D.V. Oxidative stress and antioxidant activity as the basis of senescence in maize leaves. Plant Sci. 2001, 161, 765–771. [Google Scholar] [CrossRef] [Scilit]
- Kampfenkel, K.; Vanmontagu, M.; Inze, D. Extraction and determination of ascorbate and dehydroascorbate from plant tissue. Anal. Biochem. 1995, 225, 165–167. [Google Scholar] [CrossRef] [Scilit]
- Ren, R.F.; Guo, J.Y.; Ji, Z.; Du, S.H.; Yang, X.Y. Integrated transcriptomics and metabolomics to explore the mechanisms of Elaeagnus mollis Diels seed viability decline. BMC Genom. 2025, 26, 333. [Google Scholar] [CrossRef] [Scilit]
- Han, Z.; Wang, Z.; Bi, Y.; Zong, Y.; Gong, D.; Wang, B.; Li, B.; Sionov, E.; Prusky, D. The effect of environmental pH during Trichothecium roseum (Pers.:Fr.) link inoculation of apple fruits on the host differential reactive oxygen species metabolism. Antioxidants 2021, 10, 692. [Google Scholar] [CrossRef] [Scilit]
- Davidson, N.M.; Oshlack, A. Corset: Enabling differential gene expression analysis for denovo assembled transcriptomes. Genome Biol. 2014, 15, 410. [Google Scholar] [CrossRef] [Scilit]
- Langfelder, P.; Horvath, S. WGCNA: An R package for weighted correlation network analysis. BMC Bioinf. 2008, 9, 559. [Google Scholar] [CrossRef] [Scilit]
- Xu, J.; Li, B.; Liu, Q.; Shi, Y.; Peng, J.; Jia, M.; Liu, Y. Wide-scale pollen banking of ornamental plants through cryopreservation. Cryoletters 2014, 35, 312–319. [Google Scholar]
- Chmielarz, P. Cryopreservation of dormant orthodox seeds of forest trees: Mazzard cherry (Prunus avium L.). Ann. For. Sci. 2009, 66, 405. [Google Scholar] [CrossRef] [Scilit]
- Hoekstra, F.A.; Golovina, E.A.; Buitink, J. Mechanisms of plant desiccation tolerance. Trends Plant Sci. 2001, 6, 431–438. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Karun, A.; Sajini, K.K.; Nair, M.; Kumaran, P.M.; Samsudheen, K. Cryopreservation of coconut (Cocos nucifera L.) pollen. Plant. Crops 2006, 34, 568–571. [Google Scholar]
- Chen, Y.; Wu, J.; Ma, C.; Zhang, D.; Zhou, D.; Zhang, J.; Yan, M. Metabolome and transcriptome analyses reveal changes of rapeseed in response to ABA signal during early seedling development. BMC Plant Biol. 2024, 24, 12. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, S.; Zeng, J.; Zheng, Z.; Zhou, Q.; Chen, S.; Zheng, Y.; Wan, X.; Yang, B. Comparative transcriptome analysis reveals the mechanisms underlying differential seed vigor in two contrasting peanut genotypes. Agriculture 2022, 12, 1355. [Google Scholar] [CrossRef] [Scilit]
- Gill, S.S.; Tuteja, N. Reactive oxygen species and antioxidant machinery in abiotic stress tolerance in crop plants. Plant Physiol. Biochem. 2010, 4, 909–930. [Google Scholar] [CrossRef] [Scilit]
- Kumar, K.; Raina, S.K.; Sultan, S.M. Arabidopsis MAPK signaling pathways and their cross talks in abiotic stress response. J. Plant Bioche. Biotechnol. 2020, 29, 700–714. [Google Scholar] [CrossRef] [Scilit]
- Yang, C.; Li, X.; Zhang, Y.; Jin, H. Transcriptome analysis of Populus × canadensis ‘Zhongliao1′ in response to low temperature stress. BMC Genom. 2023, 24, 77. [Google Scholar] [CrossRef] [Scilit]
- Danquah, A.; Zelicourt, D.A.; Colcombet, J.; Hirt, H. The role of ABA and MAPK signaling pathways in plant abiotic stress responses. Biotechnol. Adv. 2014, 32, 40–52. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pitzschke, A.; Schikora, A.; Hirt, H. MAPK cascade signalling networks in plant defence. Curr. Opin. Plant Biol. 2009, 12, 421–426. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chinnusamy, V.; Zhu, J.; Zhu, J.K. Cold stress regulation of gene expression in plants. Trends Plant Sci. 2007, 12, 444–451. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jia, Y.; Ding, Y.; Shi, Y.; Zhang, X.; Gong, Z.; Yang, S. The cbfs triple mutants reveal the essential functions of CBFs in cold acclimation and allow the definition of CBF regulons in Arabidopsis. New Phytol. 2016, 21, 345–353. [Google Scholar] [CrossRef] [Scilit]
- Benedict, C.; Skinner, J.S.; Meng, R.; Chang, Y.; Hurry, V. The CBF1-dependent low temperature signalling pathway, regulon and increase in freeze tolerance are conserved in Populus spp. Plant Cell Environ. 2010, 29, 1259–1272. [Google Scholar] [CrossRef] [Scilit]
- Liu, Y.; Dang, P.; Liu, L.; He, C. Cold acclimation by the CBF–COR pathway in a changing climate: Lessons from Arabidopsis thaliana. Plant Cell Rep. 2019, 3, 511–519. [Google Scholar] [CrossRef] [Scilit]
- Furuya, T.; Matsuoka, D.; Nanmori, T. Membrane rigidification functions upstream of the MEKK1-MKK2-MPK4 cascade during cold acclimation in Arabidopsis thaliana. FEBS Lett. 2014, 588, 2025–2030. [Google Scholar] [CrossRef] [Scilit]
- Eremina, M.; Rozhon, W.; Poppenberger, B. Hormonal control of cold stress responses in plants. Cell. Mol. Life Sci. 2016, 73, 797–810. [Google Scholar] [CrossRef] [Scilit]
- Song, Y.; Chen, Q.; Ci, D.; Zhang, D. Transcriptome profiling reveals differential transcript abundance in response to chilling stress in Populus simonii. Plant Cell Rep. 2013, 32, 1407–1425. [Google Scholar] [CrossRef] [Scilit]
- Emenecker, R.J.; Strader, L.C. Auxin-abscisic acid interactions in plant growth and development. Biomolecules 2020, 10, 281. [Google Scholar] [CrossRef] [Scilit]
- Soon, F.F.; Ng, L.M.; Zhou, X.E.; West, G.M.; Xu, H.E. Molecular mimicry regulates ABA signaling by SnRK2 kinases and PP2C phosphatases. Science 2011, 335, 85–88. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wu, Y.; Huang, W.; Tian, Q.; Liu, J.; Mou, H. Comparative transcriptomic analysis reveals the cold acclimation during chilling stress in sensitive and resistant passion fruit (Passiflora edulis) cultivars. PeerJ 2021, 9, e10977. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lv, X.; Li, H.; Chen, X.; Xun, X.; Guo, Z.; Yu, J.; Zhou, Y. The role of calcium-dependent protein kinase in hydrogen peroxide, nitric oxide and ABA-dependent cold acclimation. J. Exp. Bot. 2018, 69, 4127–4139. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Shu, P.; Li, Y.; Sheng, J.; Shen, L. SlMAPK3 positively regulates the ethylene production of postharvest tomato fruits and is involved in ethylene-mediated cold tolerance. J. Agric. Food Chem. 2023, 7, 6003–6013. [Google Scholar] [CrossRef] [Scilit]
- Krasensky, J.; Jonak, C. Drought, salt, and temperature stress-induced metabolic rearrangements and regulatory networks. J. Exp. Bot. 2012, 6, 1593–1608. [Google Scholar] [CrossRef] [Scilit]
- Zhang, Q.; Tang, F.; Cai, W.; Peng, B.; Ning, M.; Shan, C.; Yang, X. Chitosan treatment reduces softening and chilling injury in cold-stored Hami melon by regulating starch and sucrose metabolism. Front. Plant Sci. 2022, 13, 1096017. [Google Scholar] [CrossRef] [Scilit]
- Jiang, F.; Lv, S.; Zhang, Z.; Chen, Q.; Mai, J.; Wan, X.; Liu, P. Integrated metabolomics and transcriptomics analysis during seed germination of waxy corn under low temperature stress. BMC Plant Biol. 2023, 23, 190. [Google Scholar] [CrossRef] [Scilit]
- Ende, W.; Valluru, R. Sucrose, sucrosyl oligosaccharides, and oxidative stress: Scavenging and salvaging. J. Exp. Bot. 2009, 60, 9–18. [Google Scholar] [CrossRef] [Scilit]
- Li, J.; Hu, Y.; Hu, J.; Xie, Q.; Chen, X.; Qi, X. Sucrose synthase: An enzyme with multiple roles in plant physiology. J. Plant Physiol. 2024, 303, 154352. [Google Scholar] [CrossRef] [Scilit]
- Kumar, R.; Mukherjee, S.; Ayele, B.T. Molecular aspects of sucrose transport and its metabolism to starch during seed development in wheat: A comprehensive review. Biotechnol. Adv. 2018, 36, 954–967. [Google Scholar] [CrossRef] [Scilit]
- Albrecht, G.; Mustroph, A. Localization of sucrose synthase in wheat roots: Increased in situ activity of sucrose synthase correlates with cell wall thickening by cellulose deposition under hypoxia. Planta 2003, 217, 252–260. [Google Scholar] [CrossRef] [Scilit]
- Maraña, C.; García-Olmedo, F.; Carbonero, P. Differential expression of two types of sucrose synthase-encoding genes in wheat in response to anaerobiosis, cold shock and light. Gene 1990, 88, 167–172. [Google Scholar] [CrossRef] [Scilit]
- Wen, B. Cytological and physiological changes related to cryotolerance in recalcitrant Livistona chinensis embryos during seed development. Protoplasma 2011, 24, 483–491. [Google Scholar] [CrossRef] [Scilit]
- Sengupta, S.; Datta, M.; Datta, S. β-glucosidase: Structure, function and industrial applications. Glycoside Hydrolases 2023, 97–120. [Google Scholar] [CrossRef] [Scilit]
- Jaspers, P.; Brosché, M.; Overmyer, K.; Kangasjär, J. The transcription factor interacting protein RCD1 contains a novel conserved domain. Plant Signal. Behav. 2010, 5, 78–80. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Atkinson, N.J.; Urwin, P.E. The interaction of plant biotic and abiotic stresses: From genes to the field. J. Exp. Bot. 2012, 63, 3523–3543. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Huang, X.; Liang, Y.; Zhang, B.; Song, X.; Li, Y.; Li, C.; Qin, Z.; Li, D.; Wei, J.; Wu, J. Comparative transcriptome analysis reveals potential gene modules associated with cold tolerance in sugarcane (Saccharum officinarum L.). J. Plant Growth Regul. 2022, 41, 2614–2628. [Google Scholar] [CrossRef] [Scilit]
- Ritonga, F.N.; Chen, S. Physiological and molecular mechanism involved in cold stress tolerance in plants. Plants 2020, 9, 560. [Google Scholar] [CrossRef] [Scilit]
- Liu, J.; Shi, Y.; Yang, S. Insights into the regulation of C-repeat binding factors in plant cold signaling. J. Integr. Plant Biol. 2018, 60, 780–795. [Google Scholar] [CrossRef] [Scilit]
- Park, S.; Lee, C.; Doherty, C.J.; Gilmour, S. Regulation of the Arabidopsis CBF regulon by a complex low-temperature regulatory network. Plant J. 2015, 8, 193–207. [Google Scholar] [CrossRef] [Scilit]
- Tang, B.; Zhang, B.H.; Mo, C.Y.; Fu, W.Y.; Yang, W.; Wang, Q.Q.; Ao, N.; Qu, F.; Tan, G.F.; Tao, L. Comparative transcriptomics reveal the mechanisms underlying the glucosinolate metabolic response in leaf Brassica juncea L. under cold stress. Agronomy 2023, 13, 1922. [Google Scholar] [CrossRef] [Scilit]
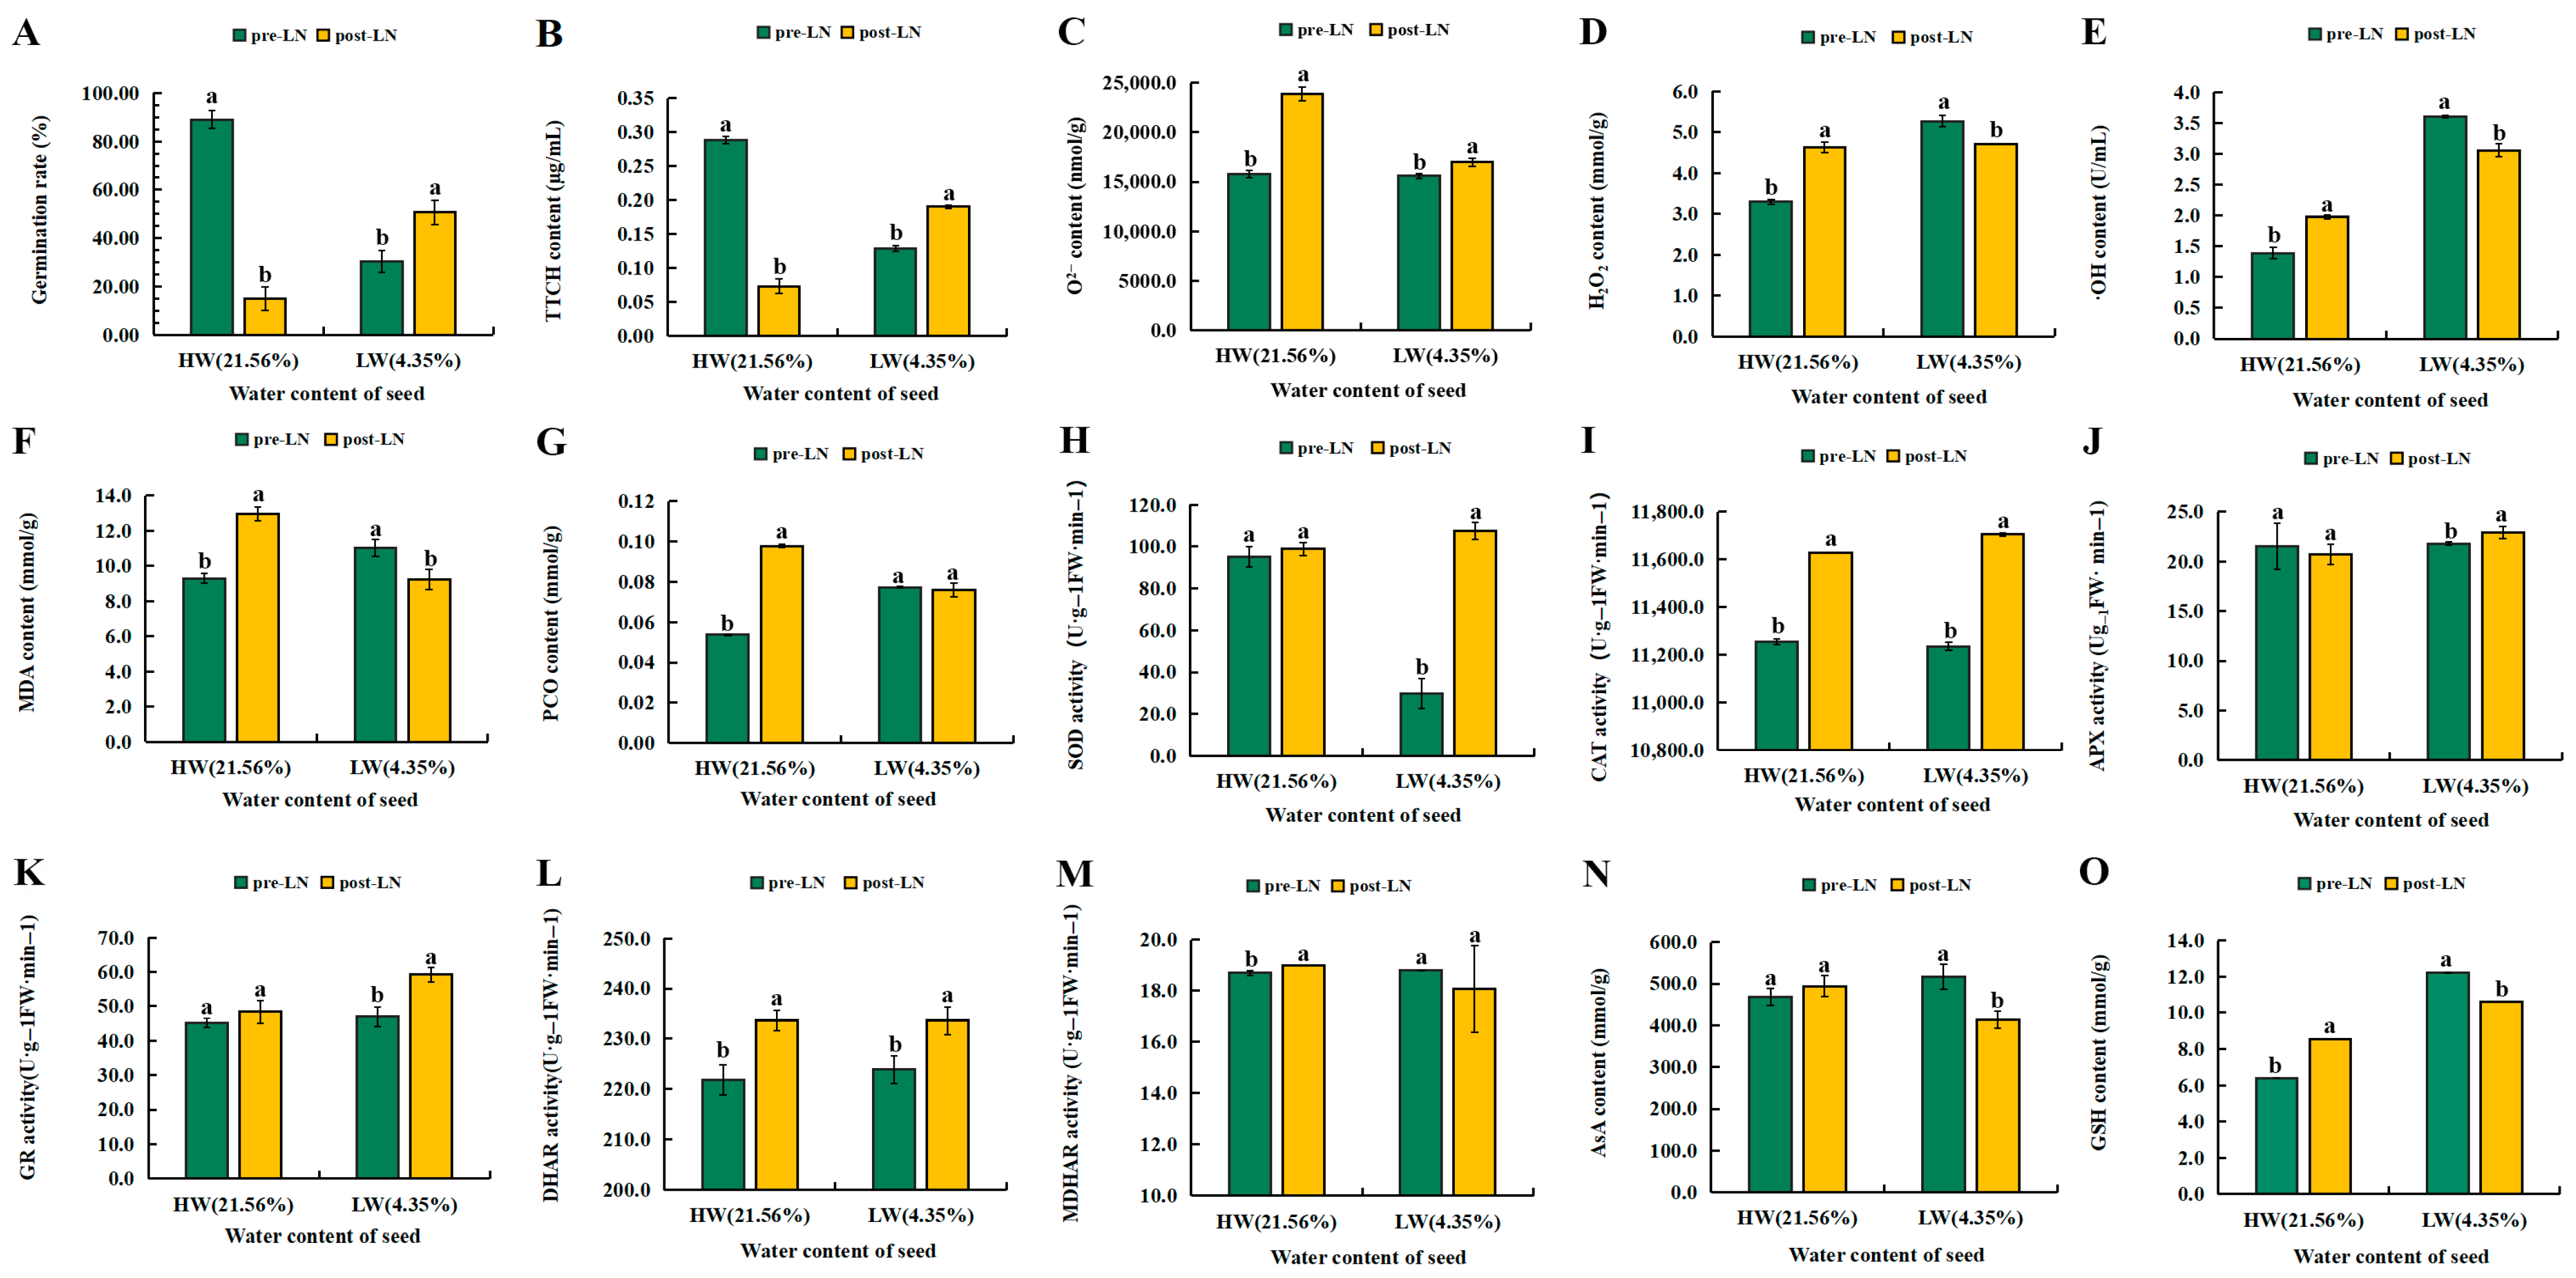
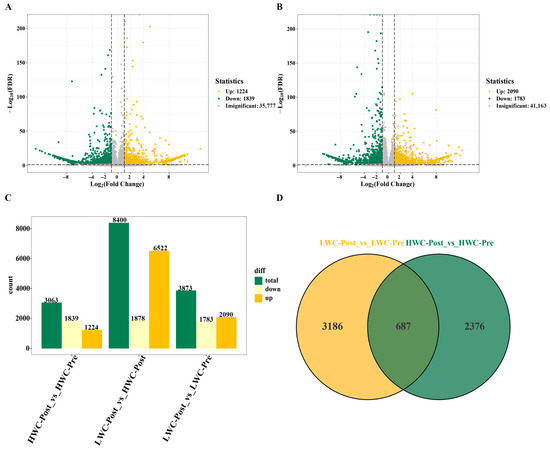
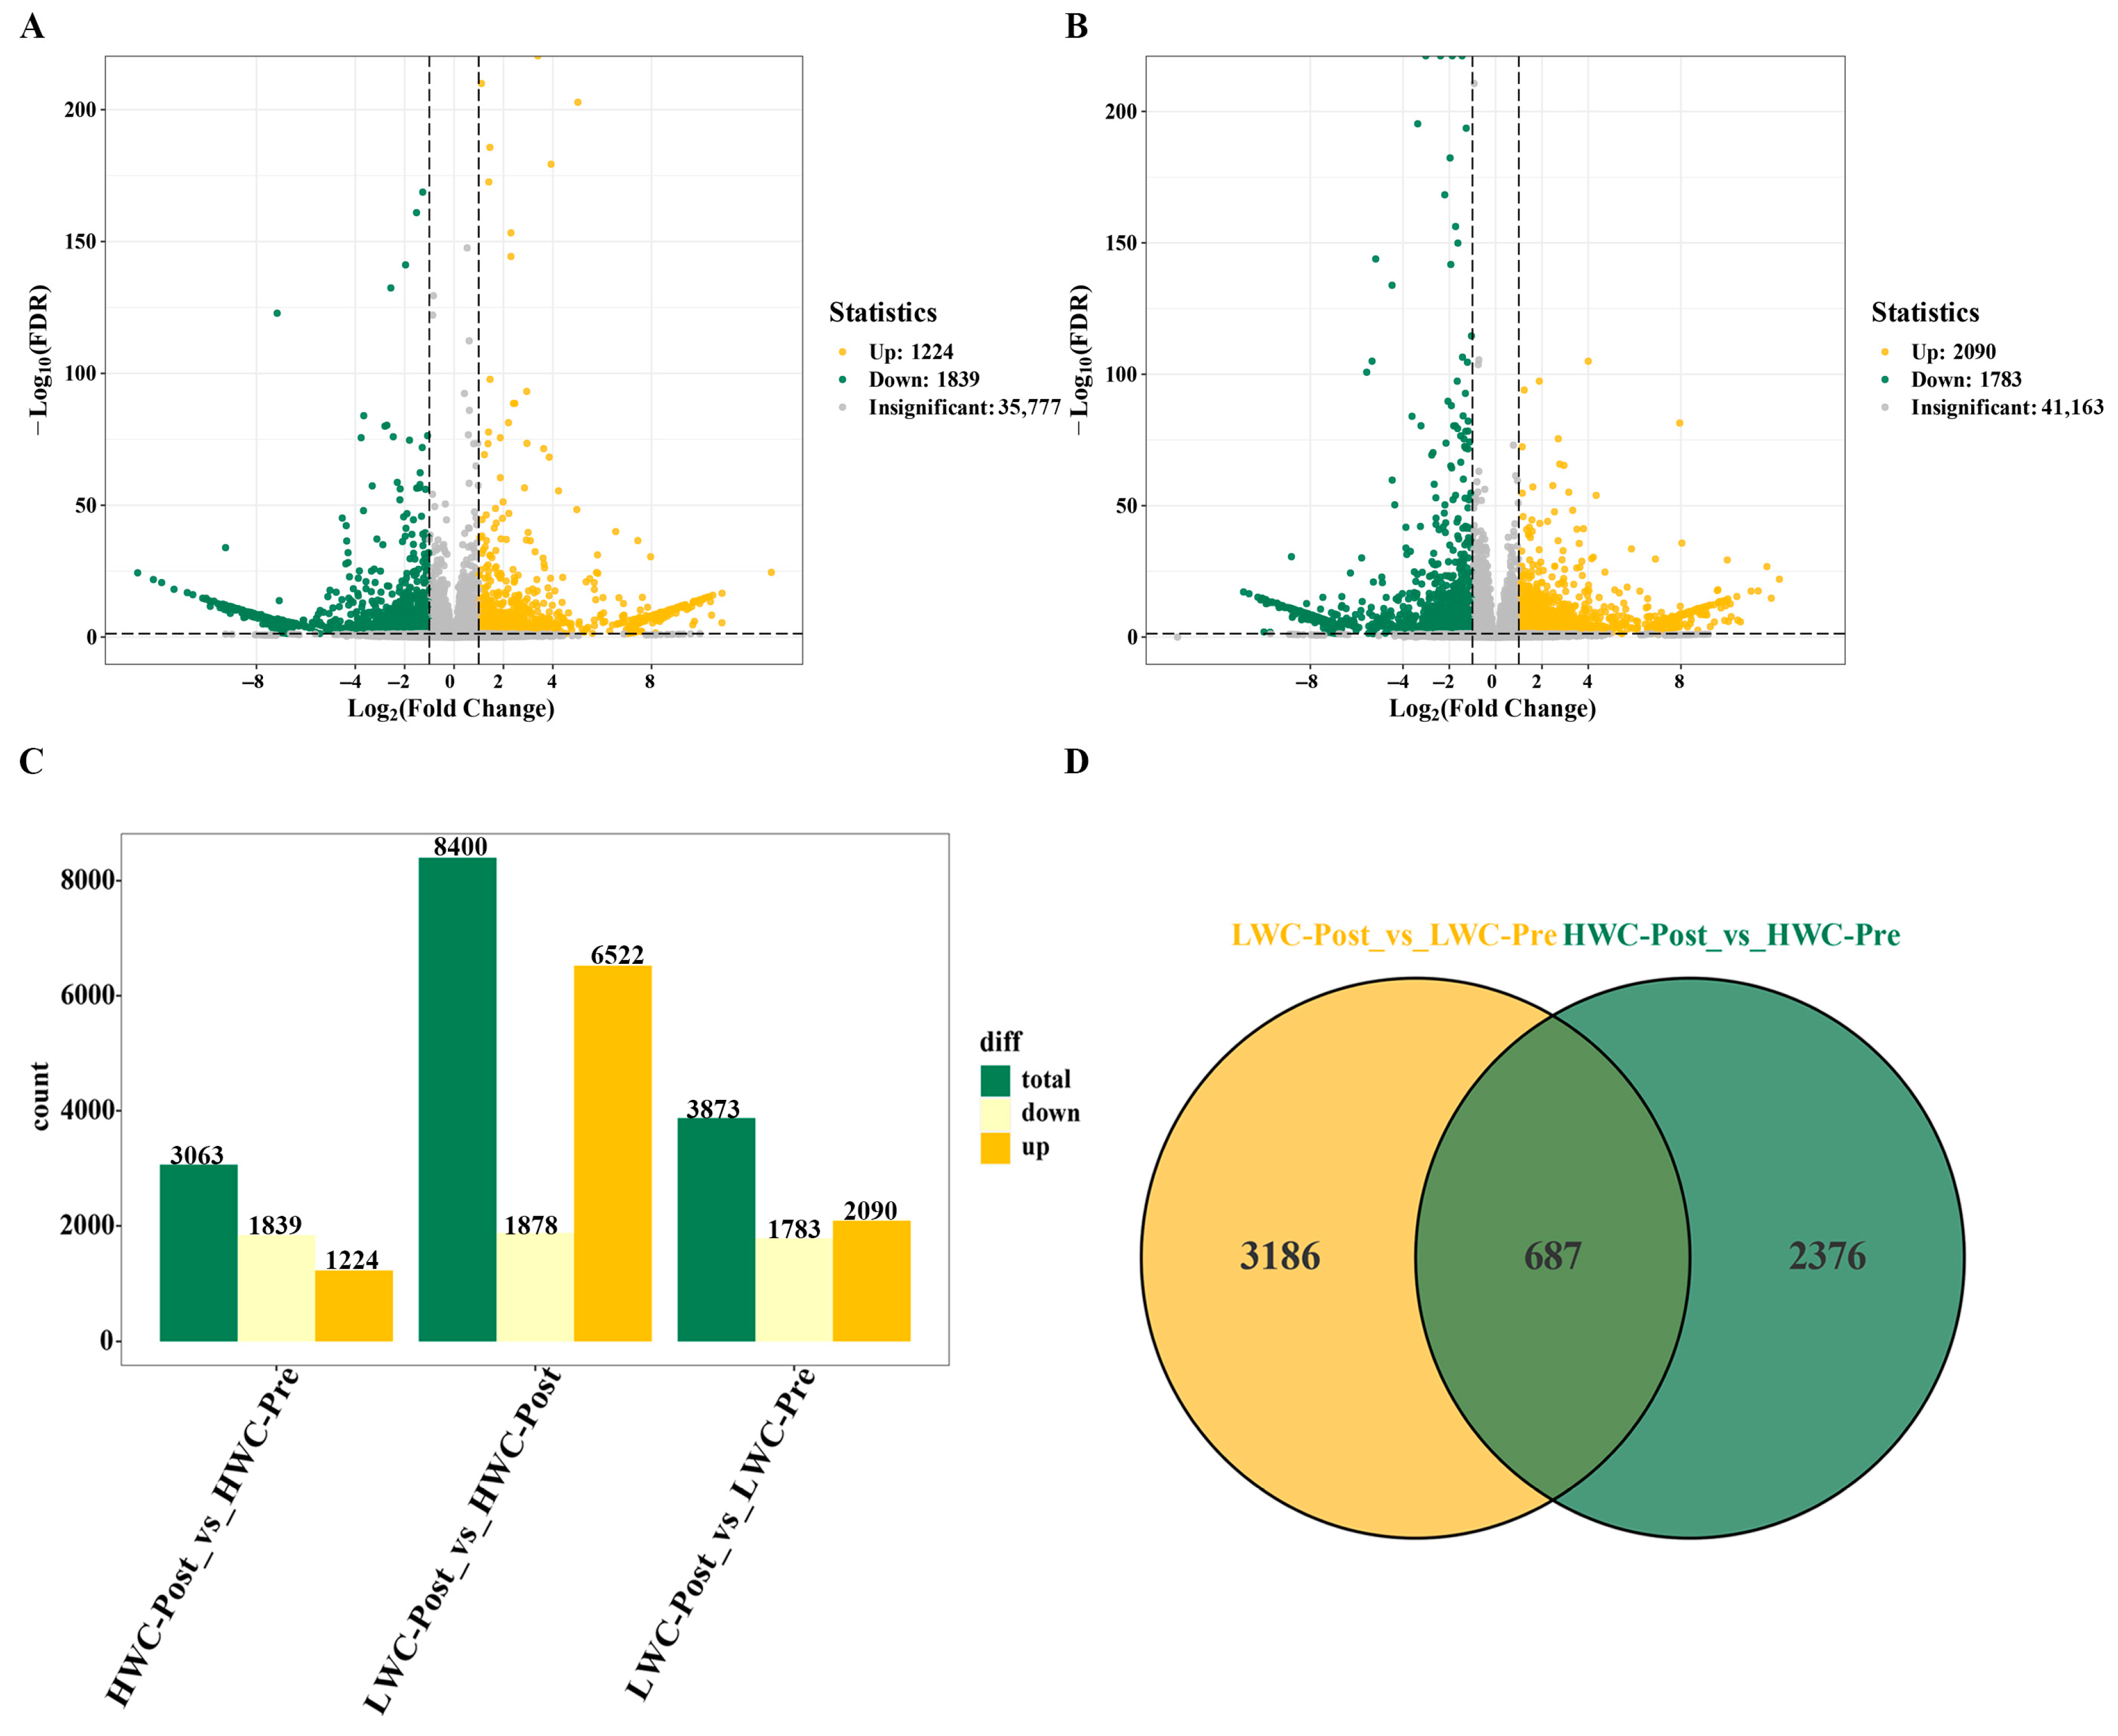
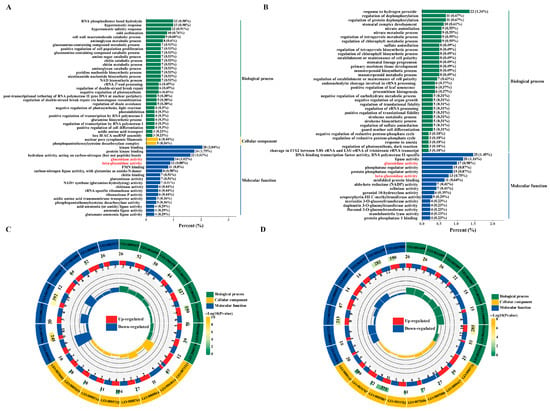
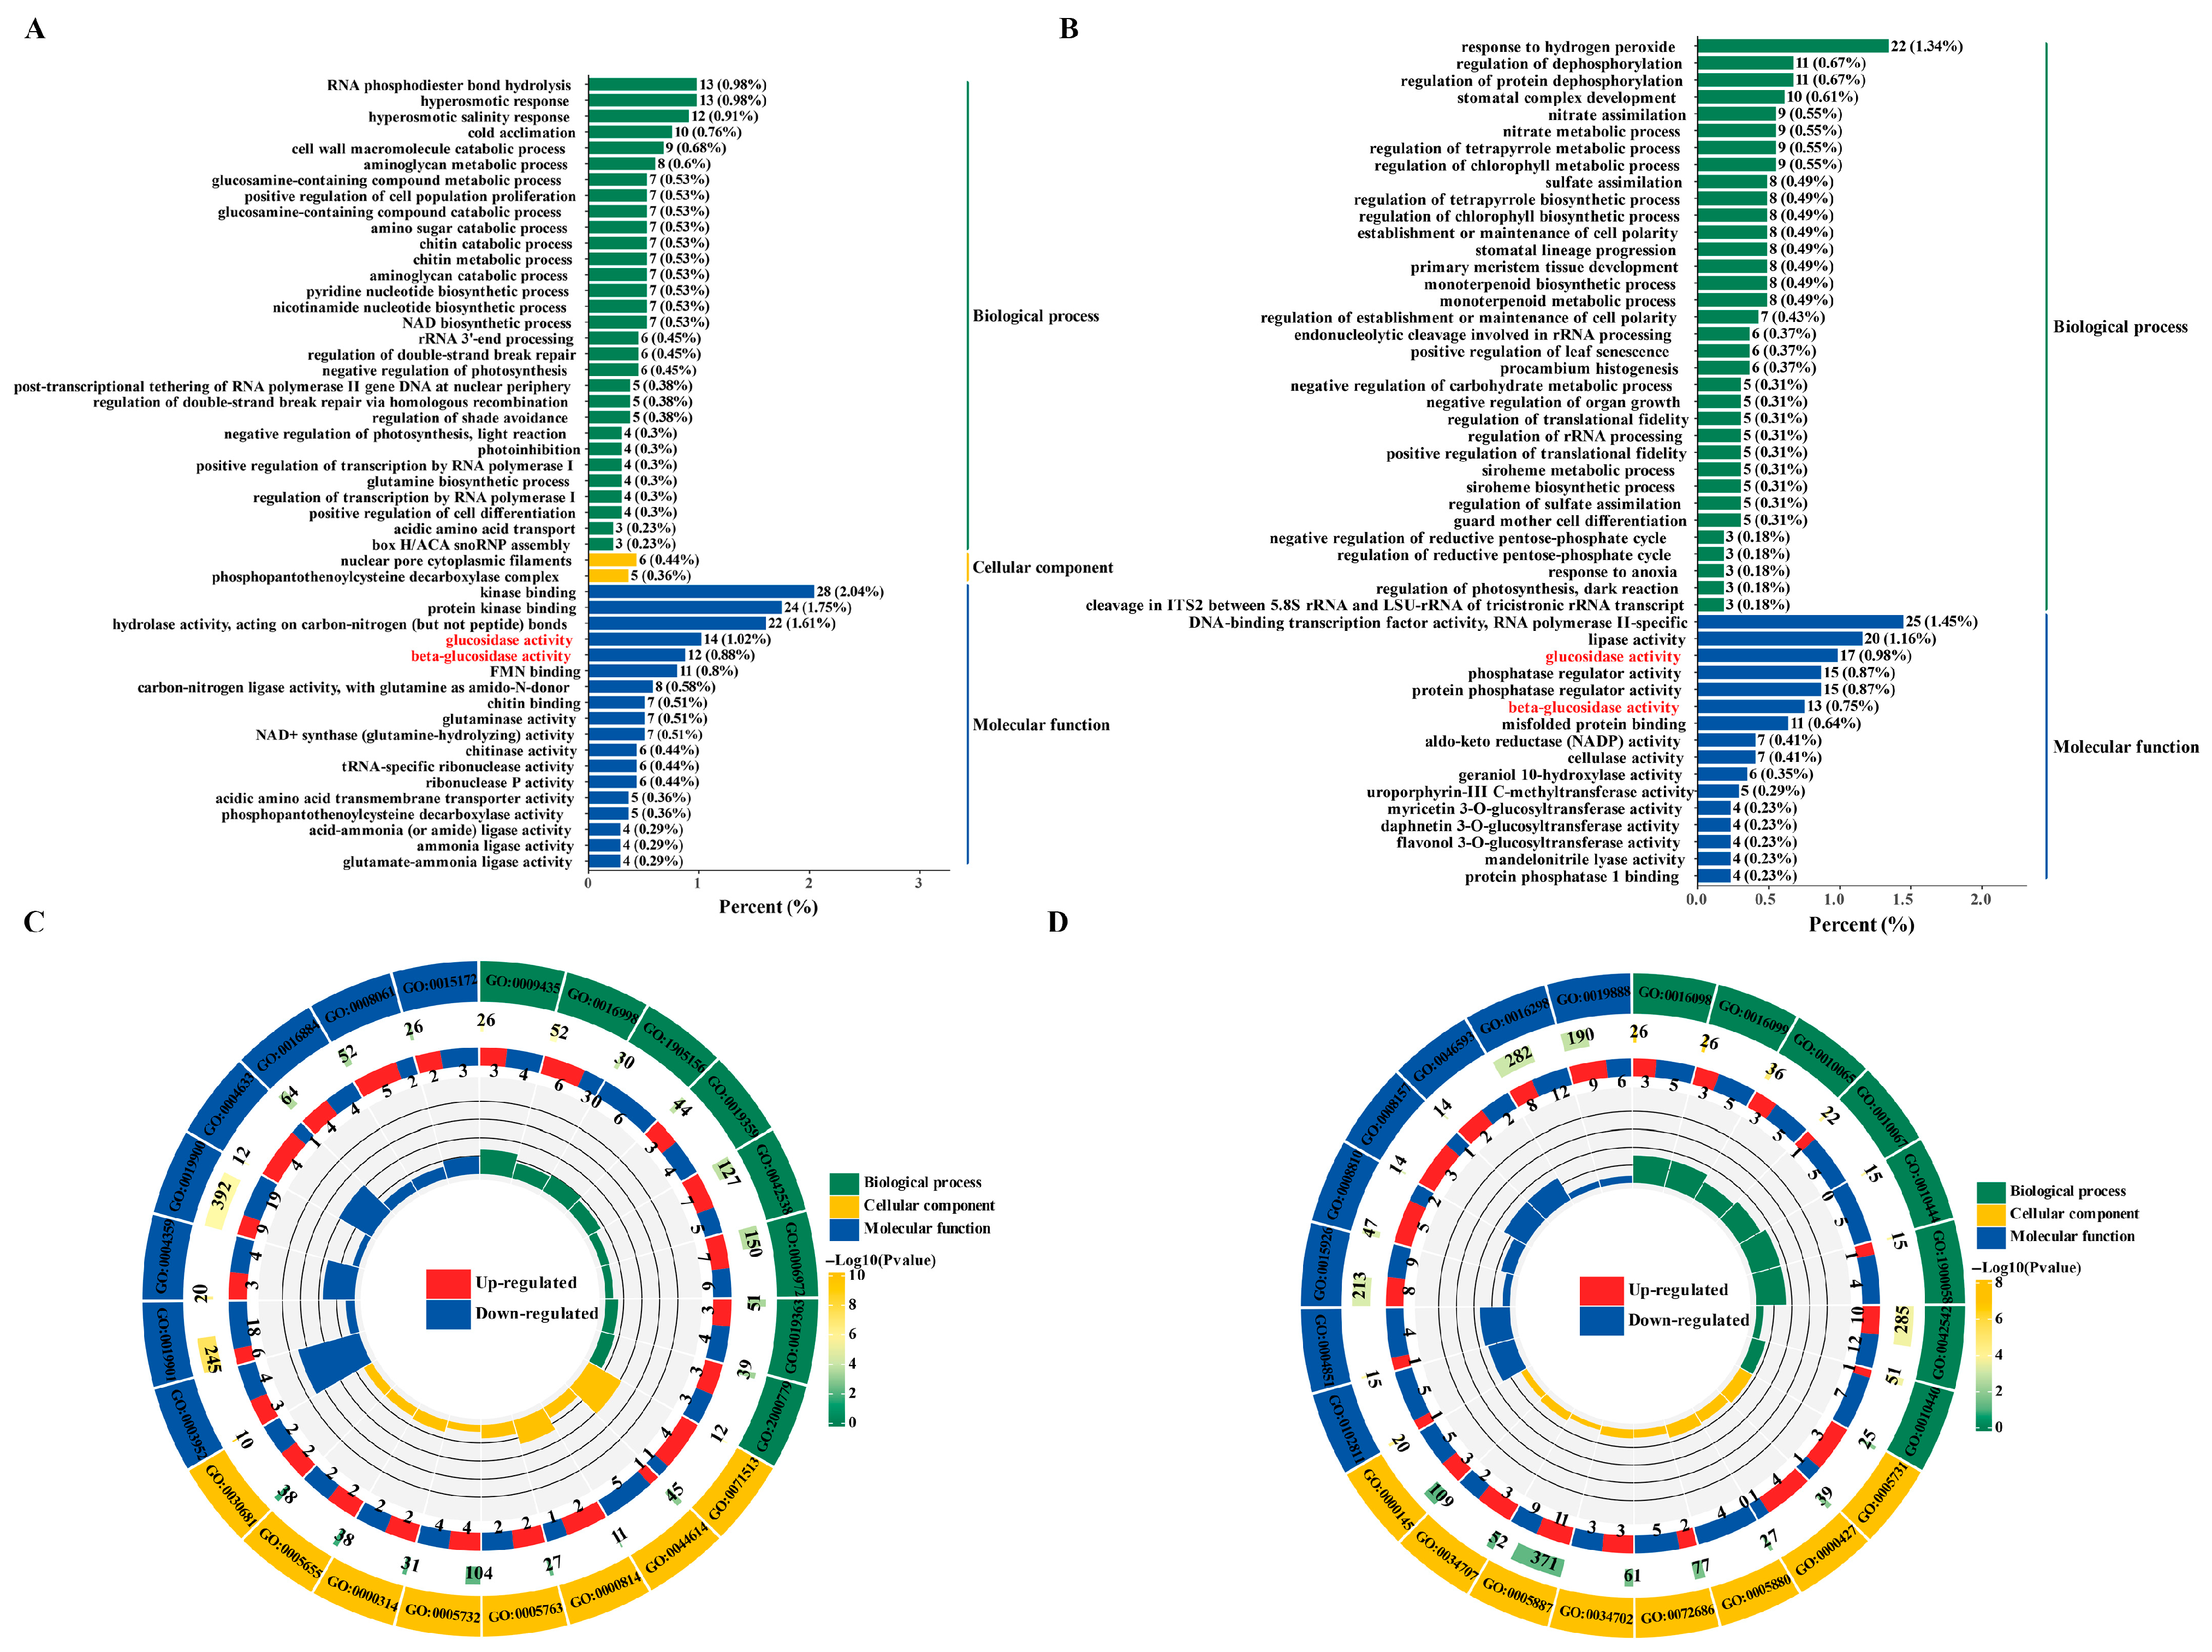
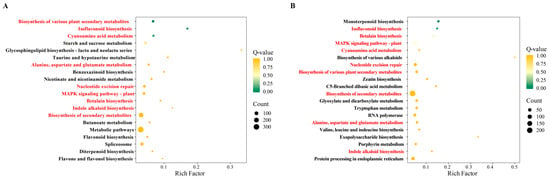
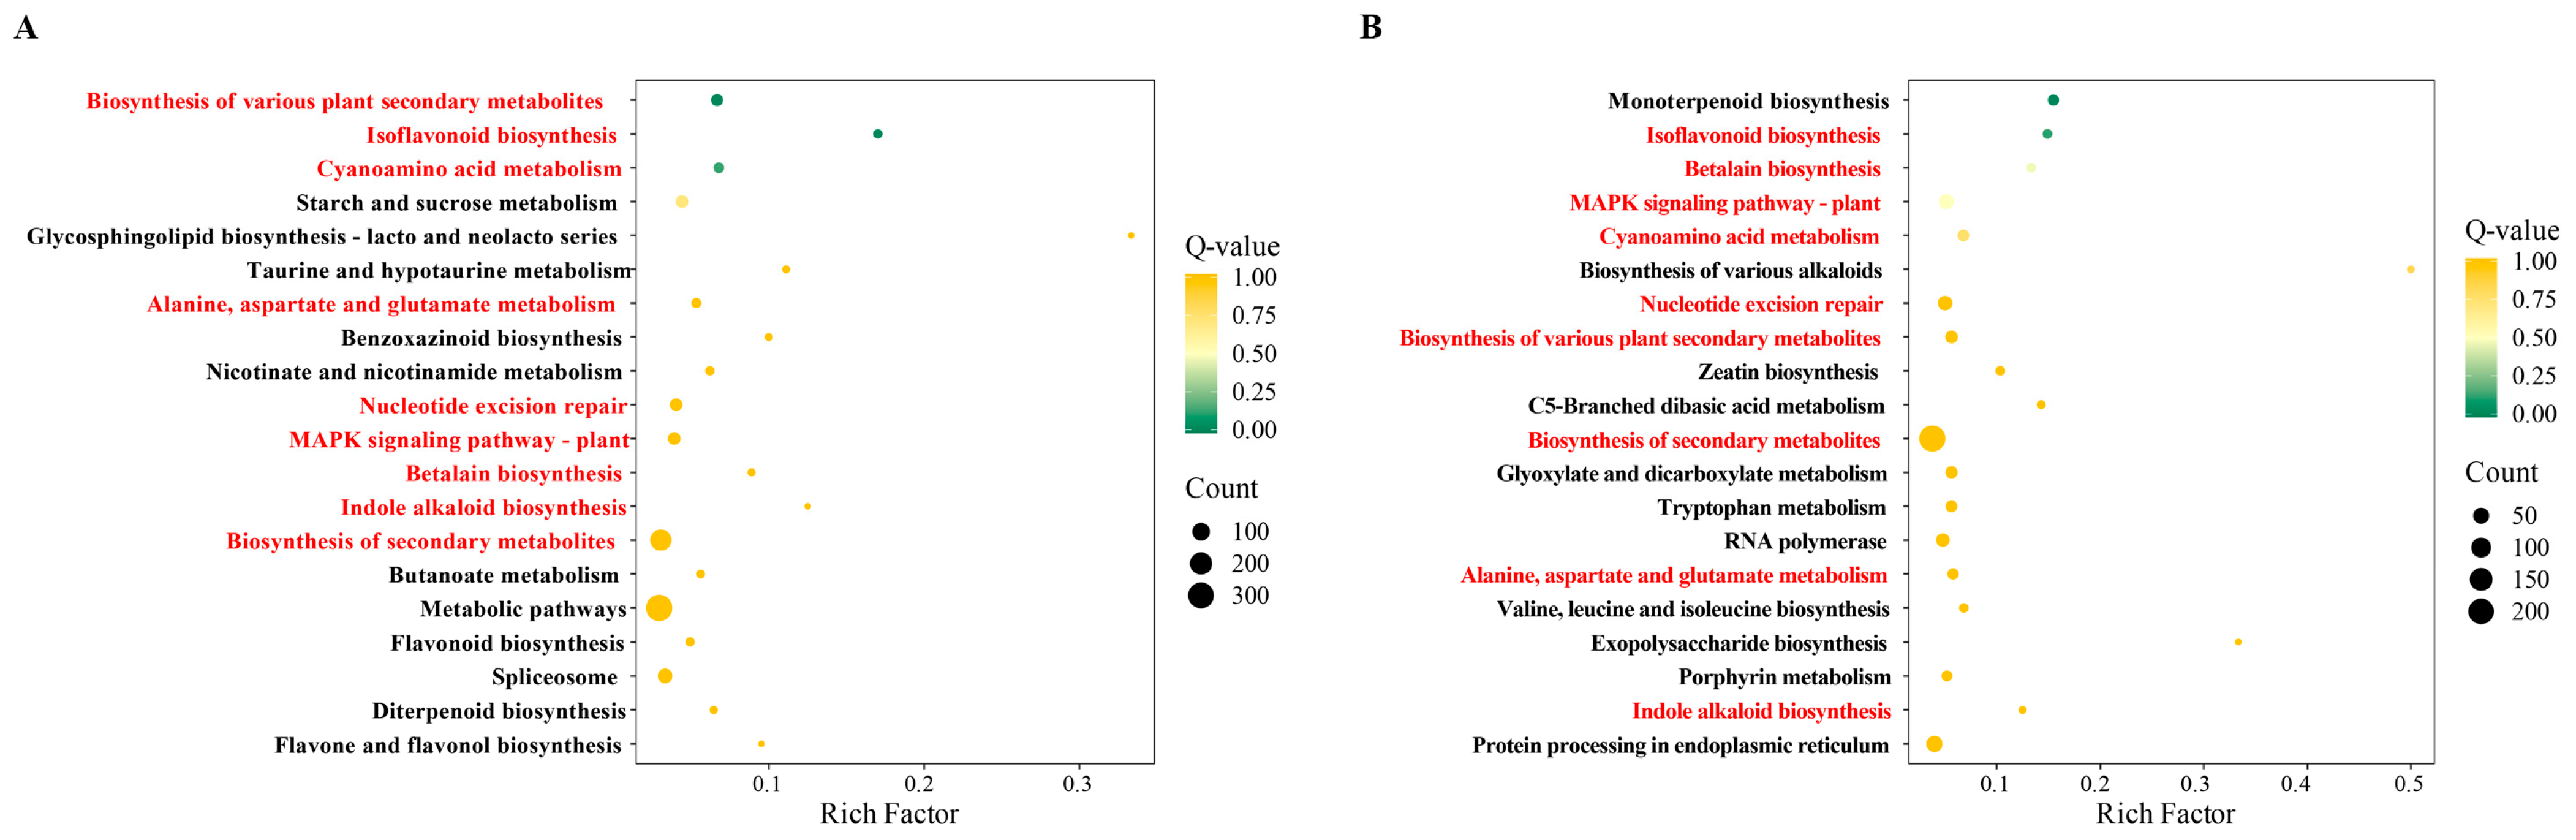
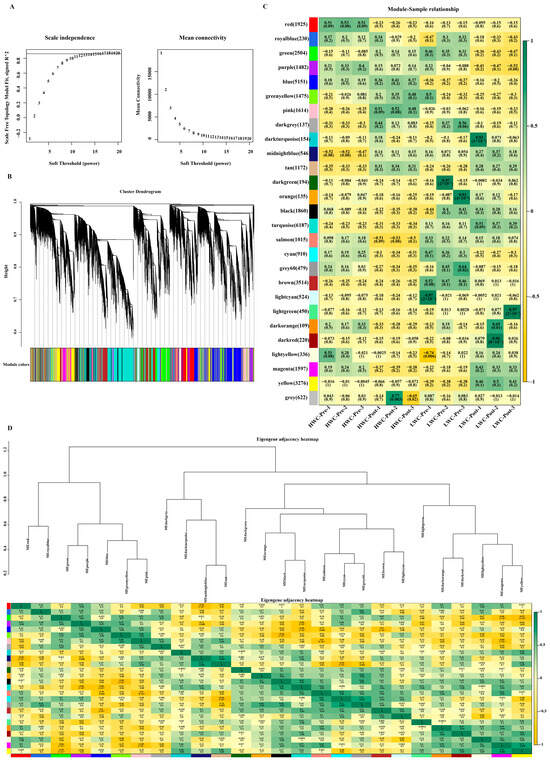
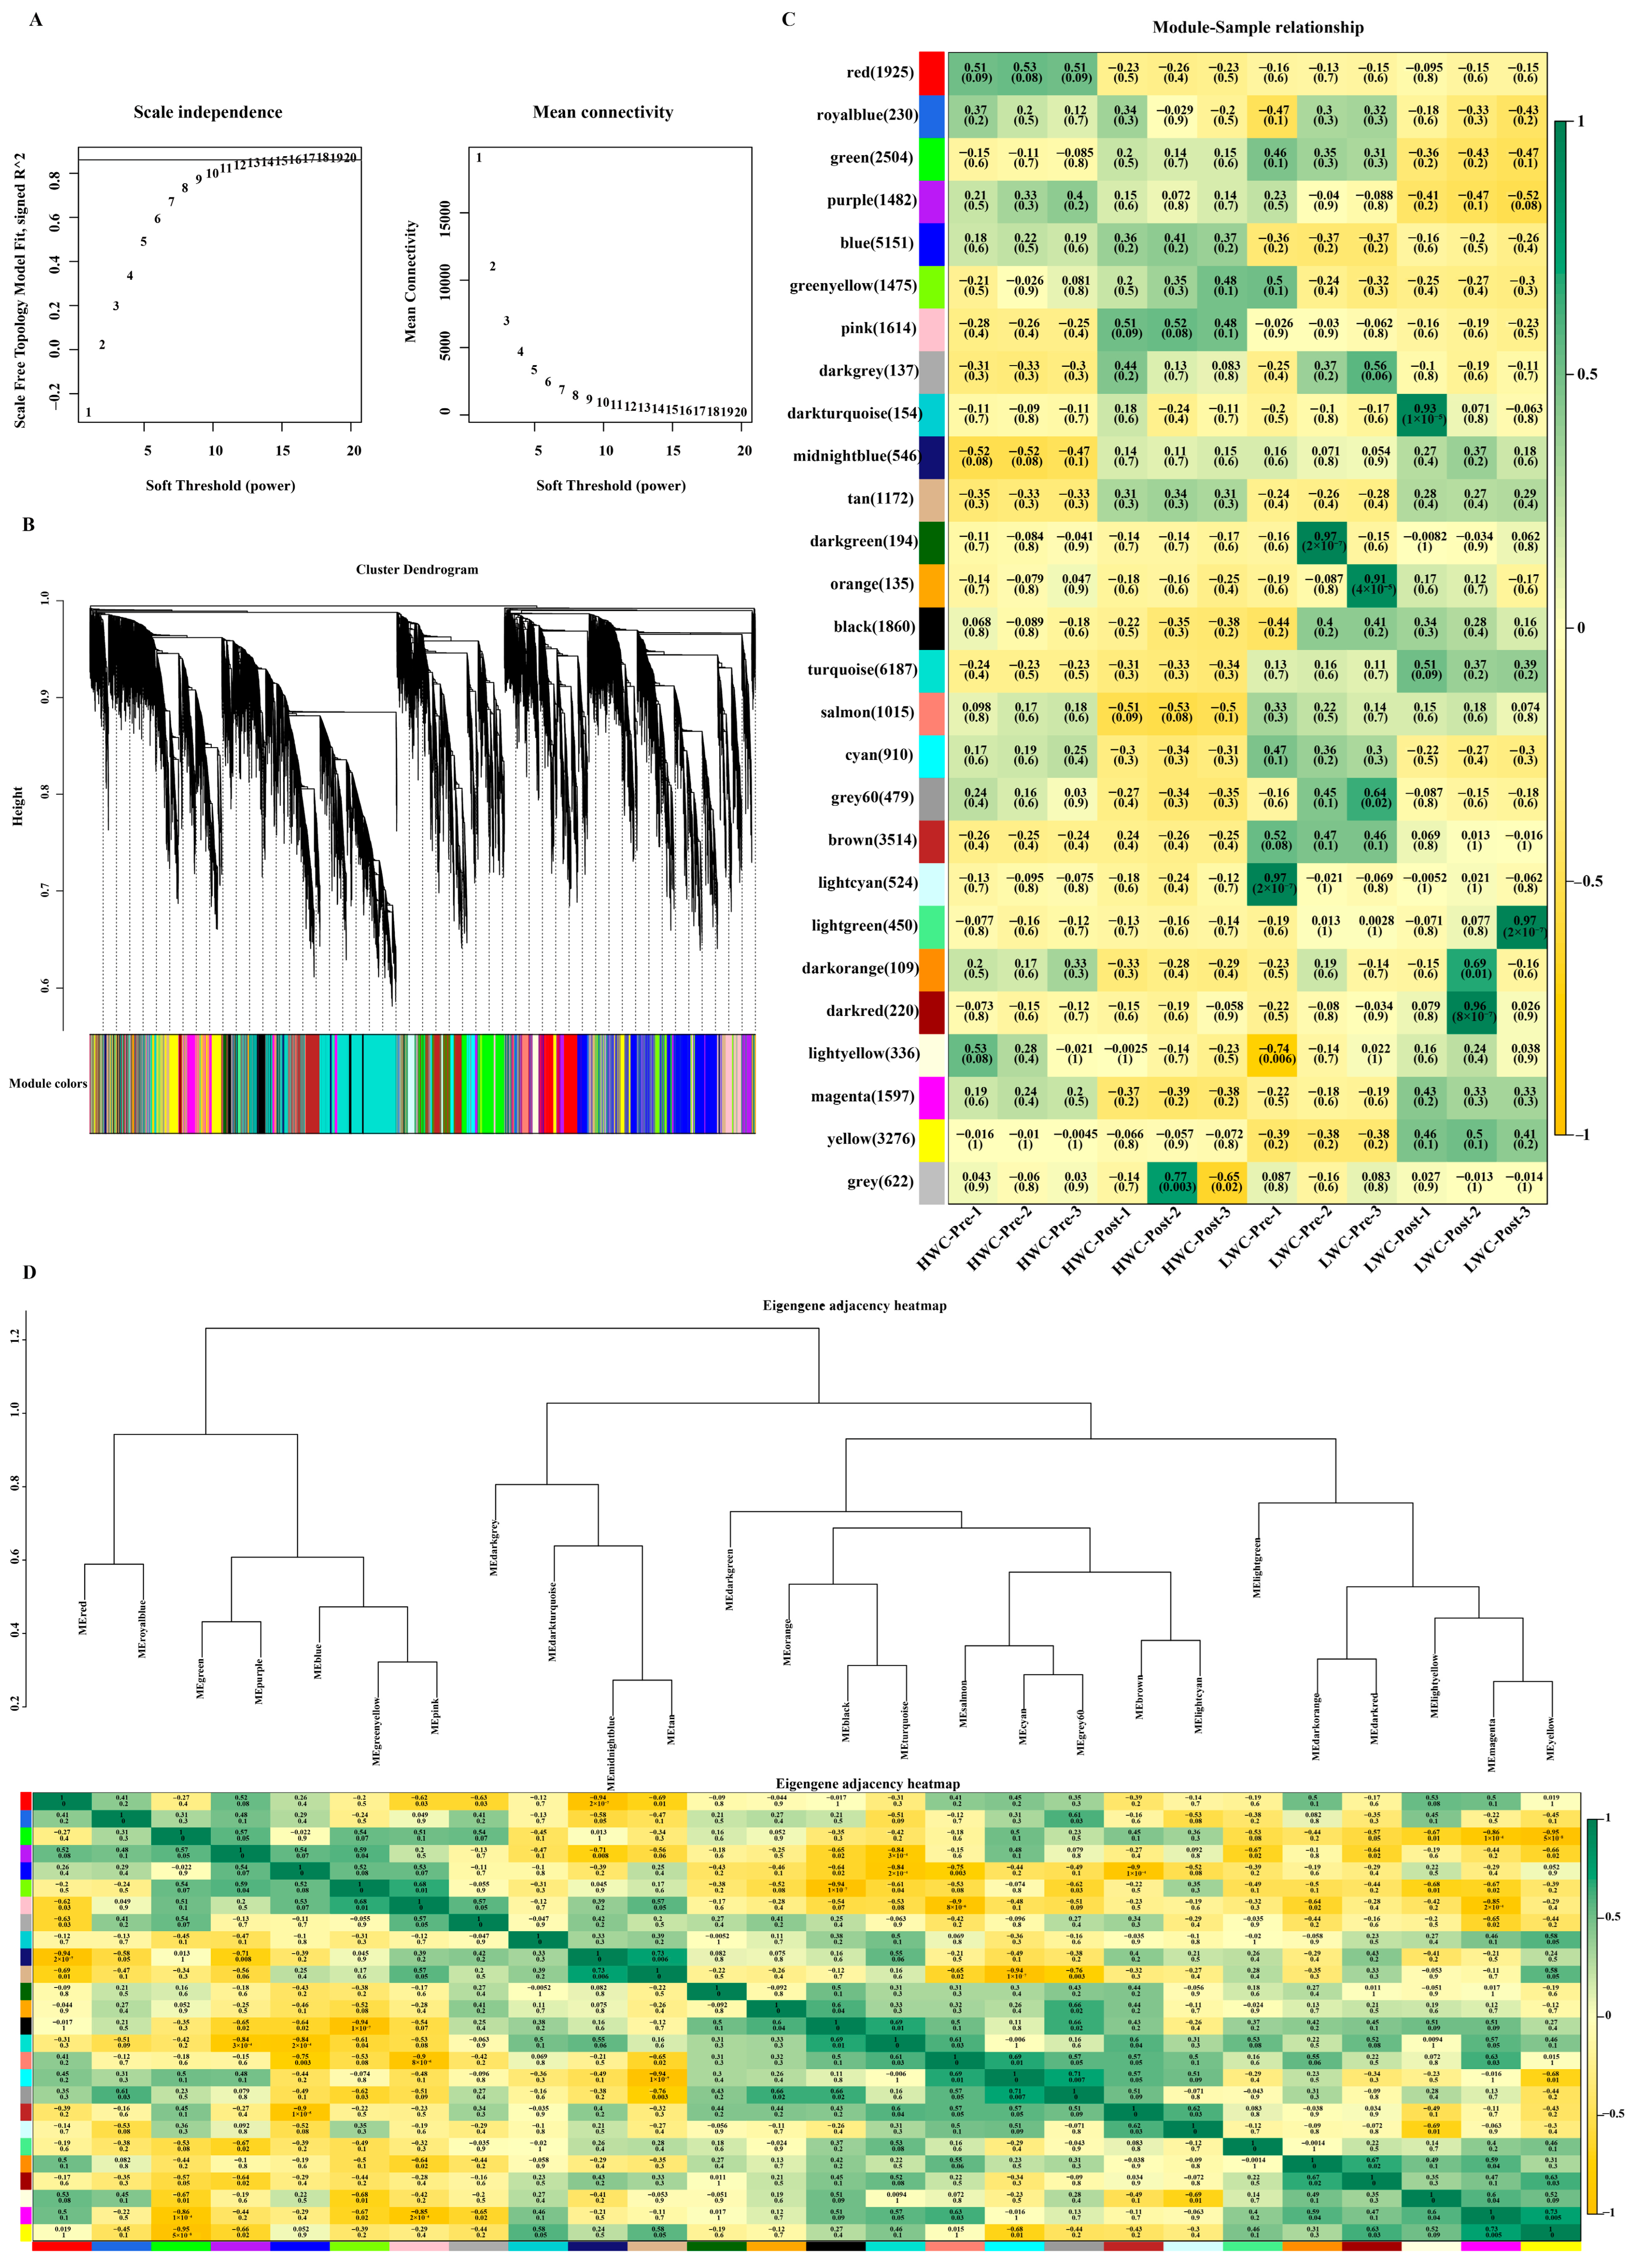
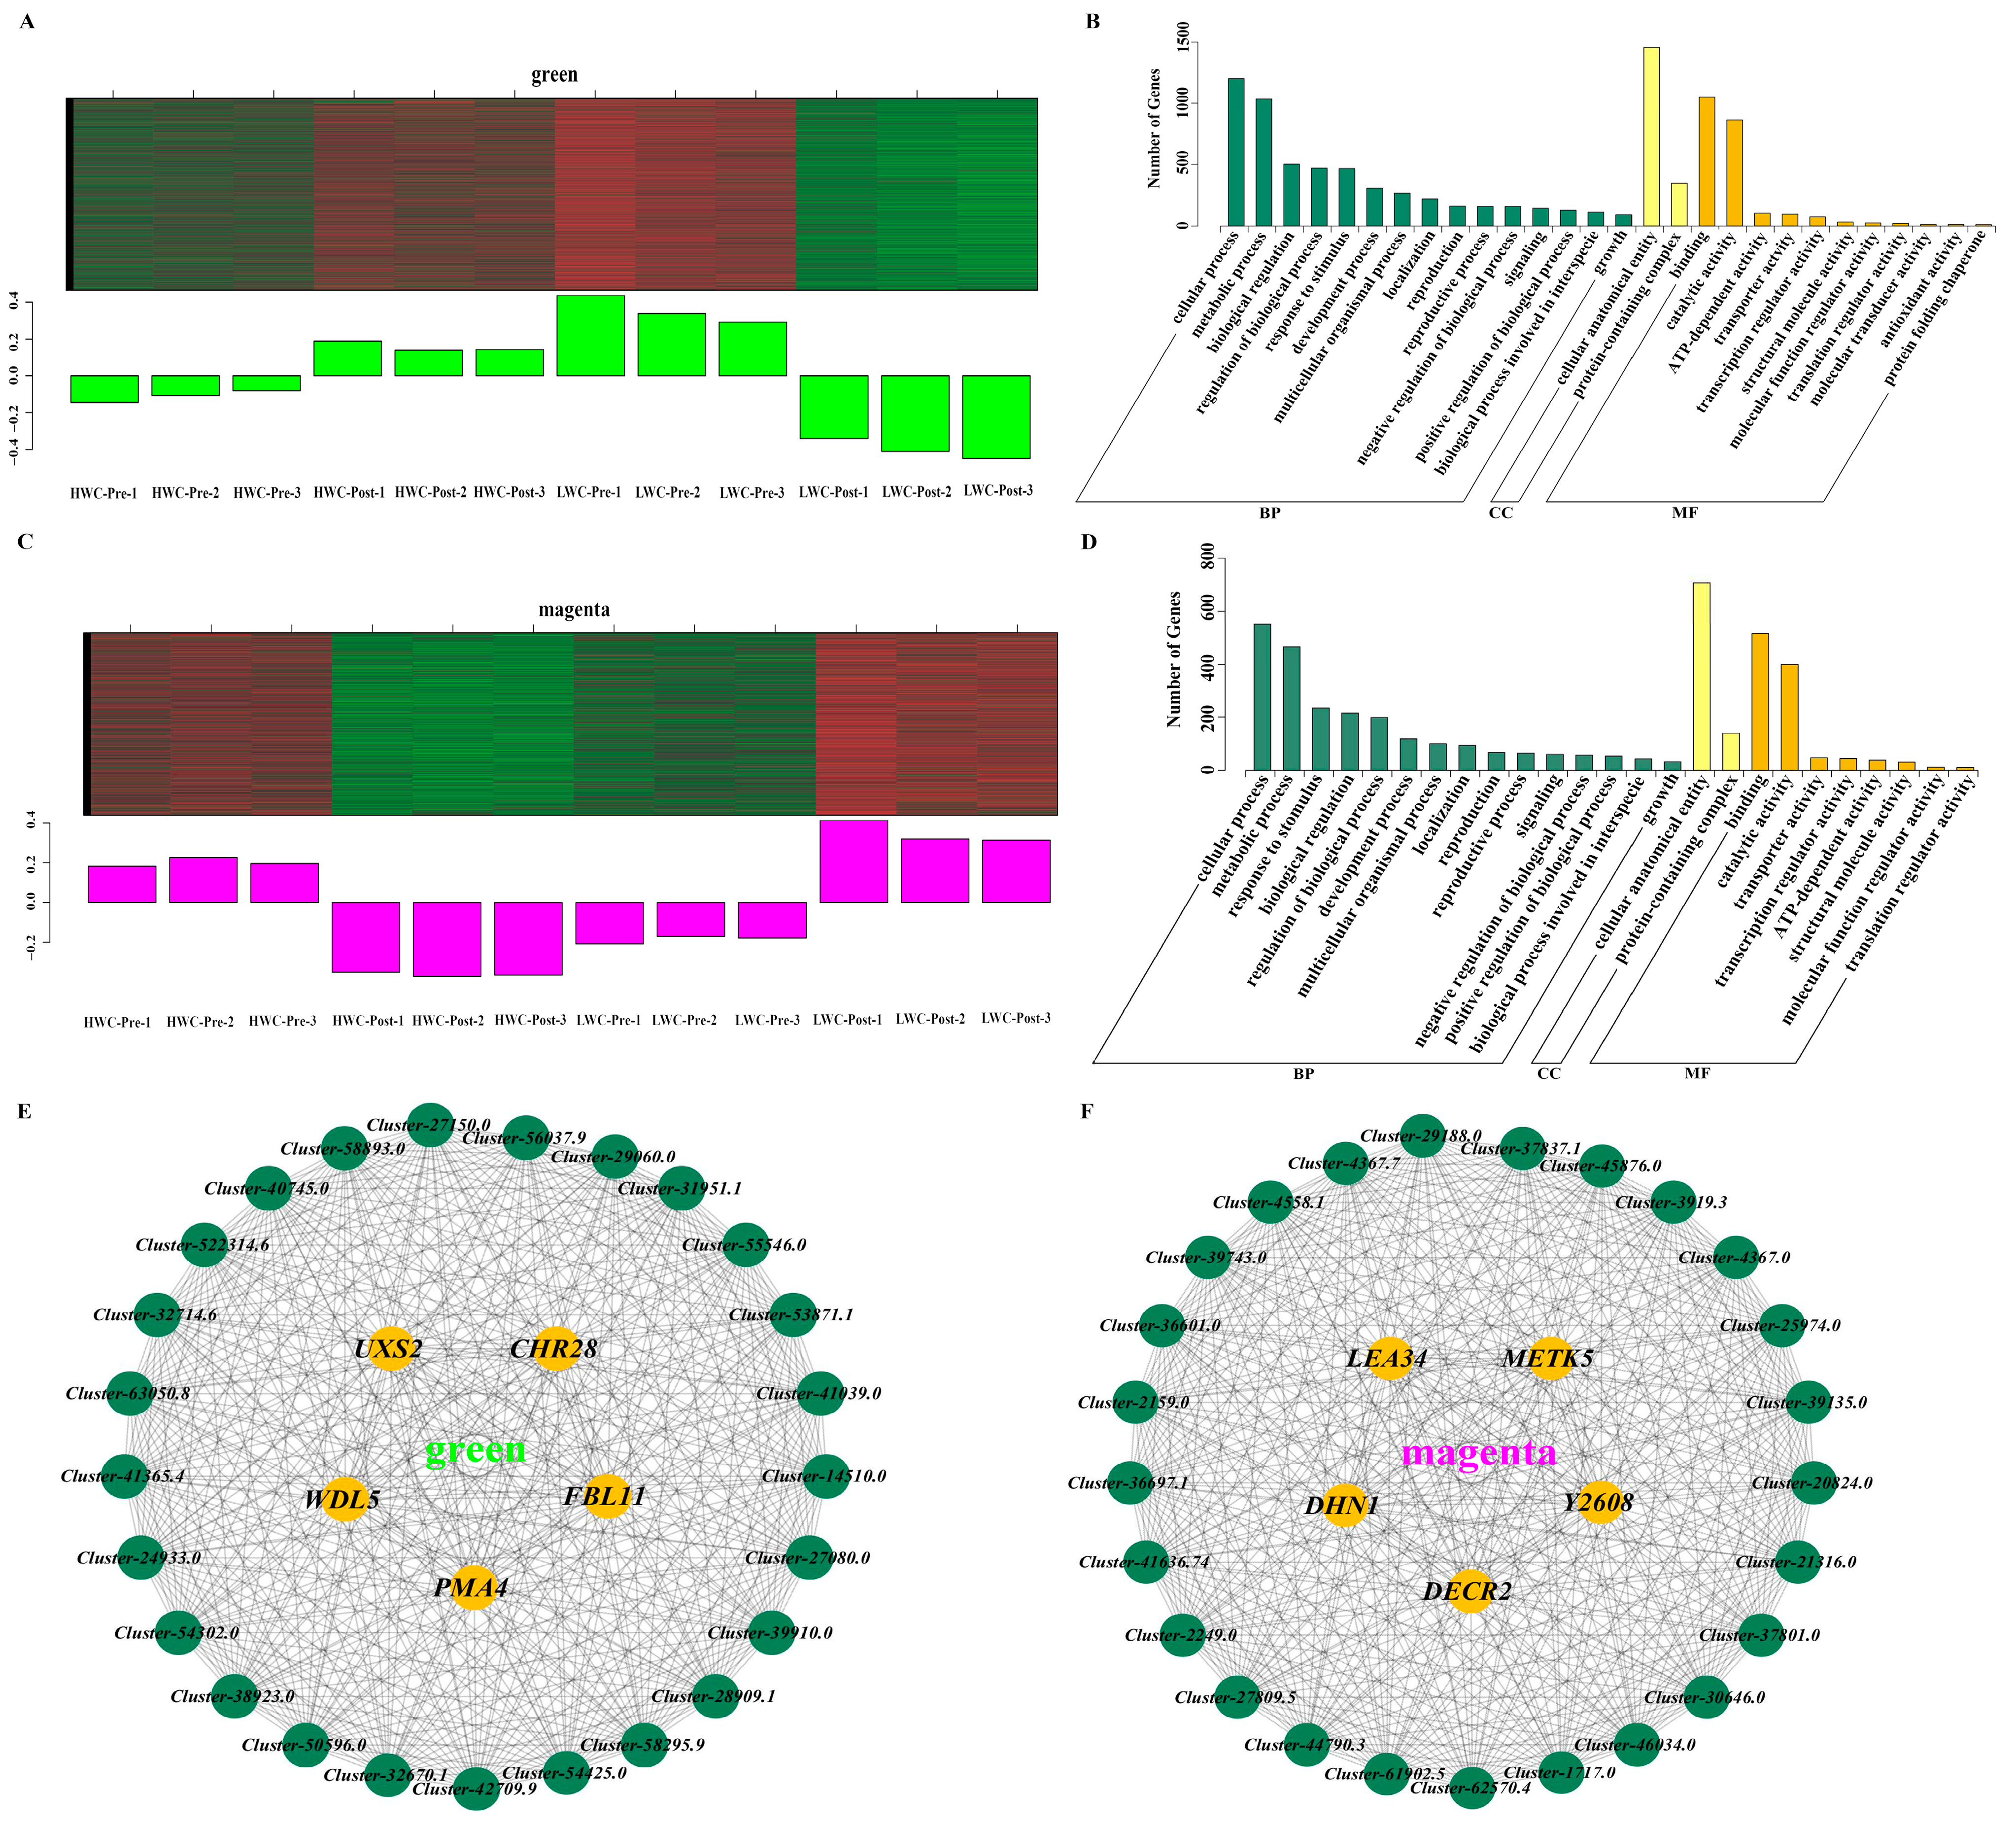
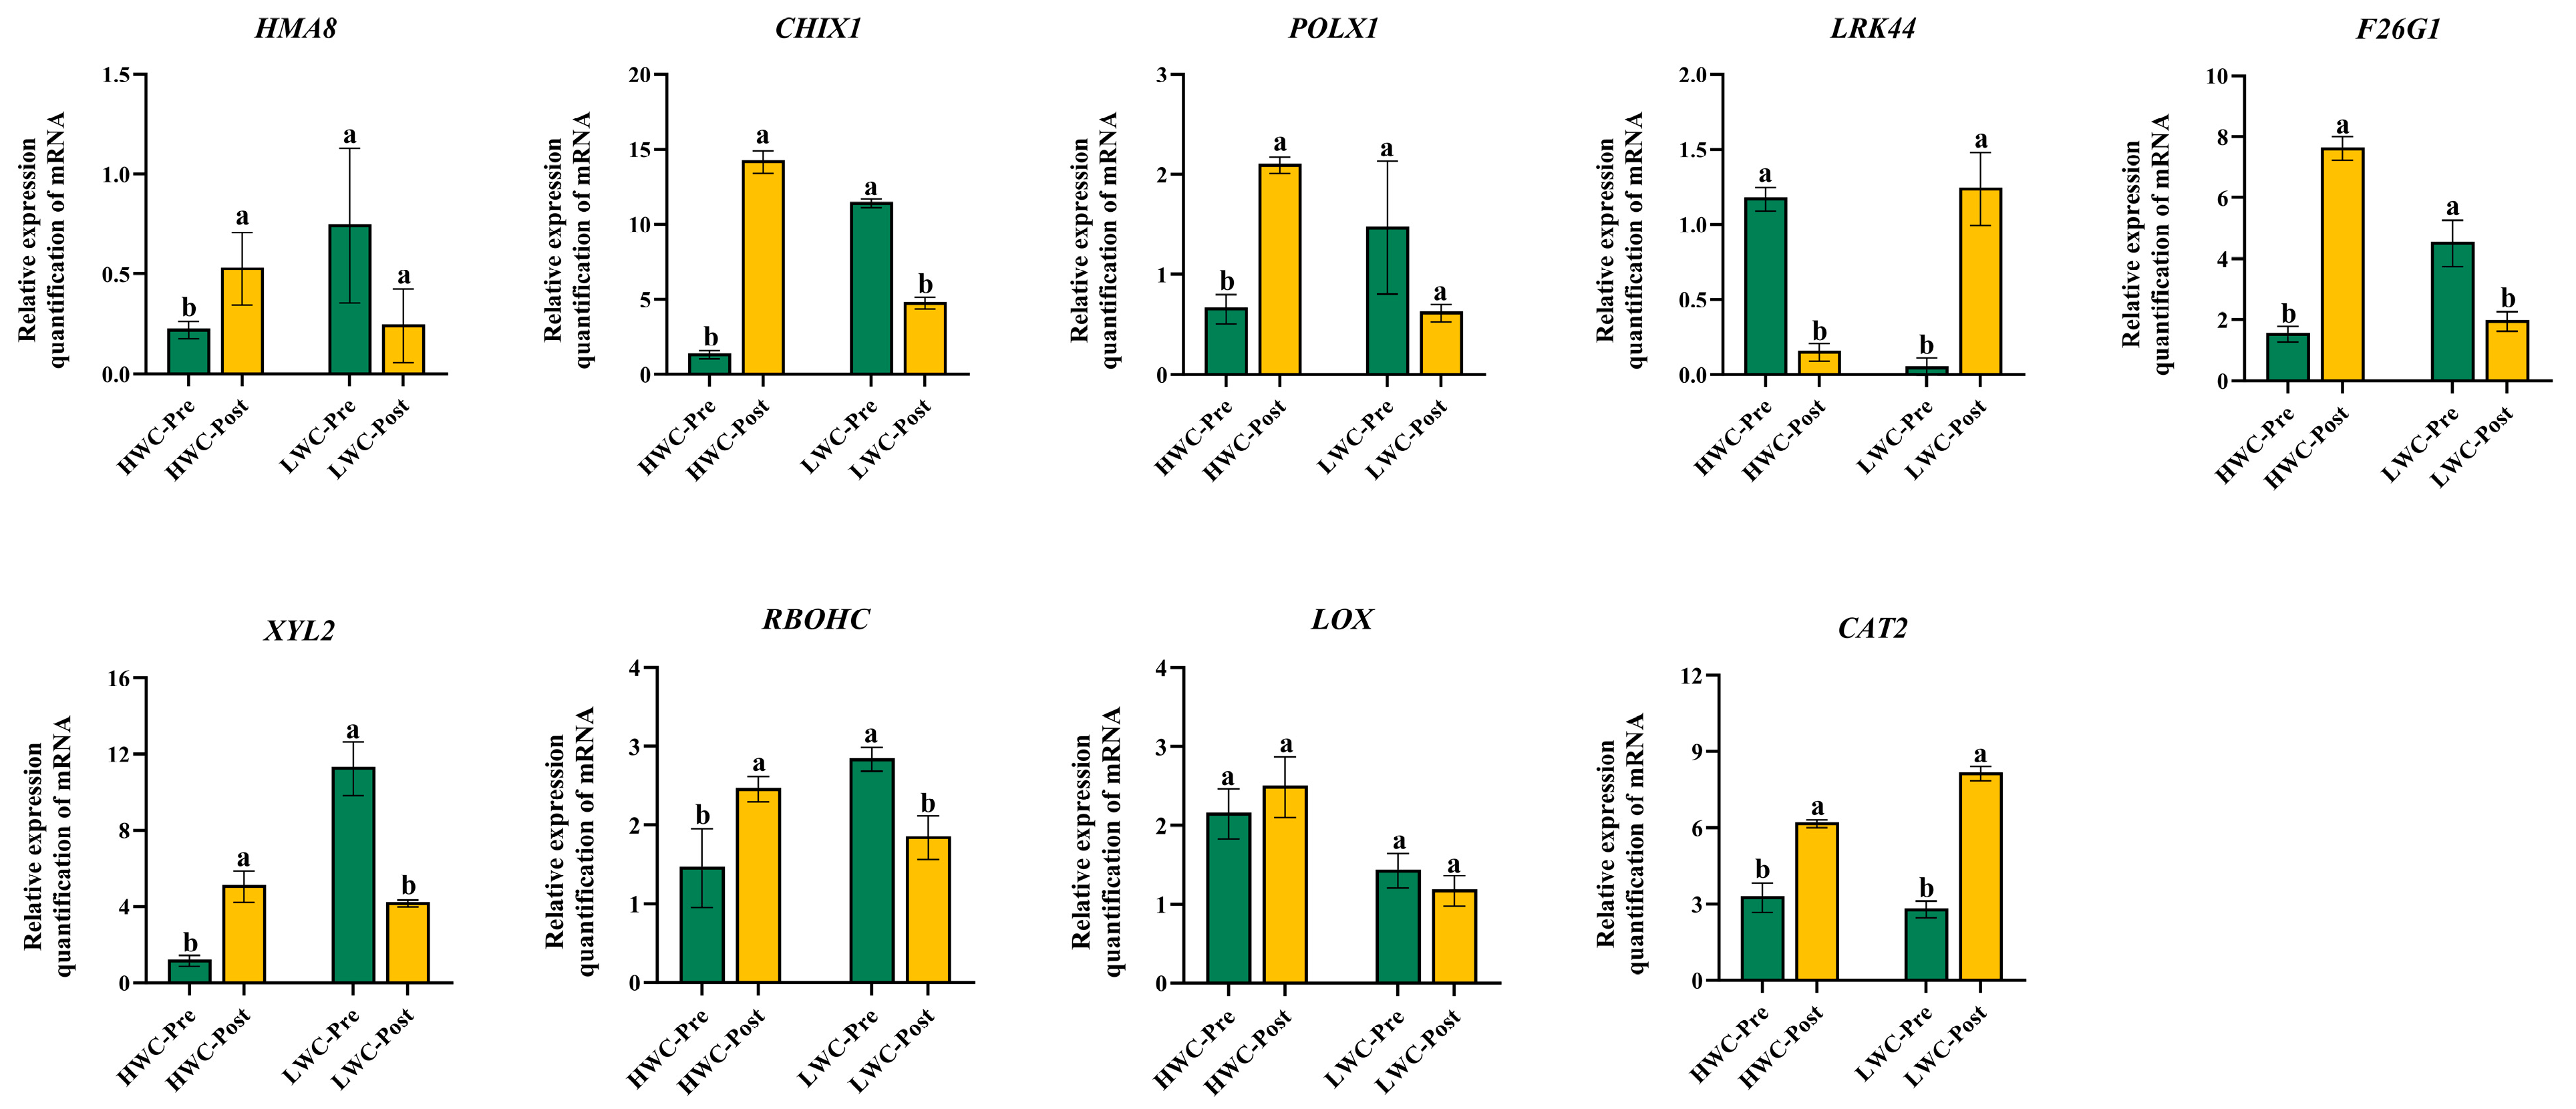
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2025 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).