


Abstract
The use of mycorrhizal fungi to enhance orchid seed germination and seedling growth is a promising approach for orchid propagation and conservation, but practical applications remain limited. In this study, we developed a direct seeding technique based on mycorrhizal symbiosis using Dendrobium officinale. Seeds were inoculated with two fungal strains, Serendipita officinale (SO) and Serendipita indica (SI), individually or in combination, and cultivated on three substrates to identify optimal fungus–substrate combinations. SO achieved the highest germination rate (52.9 ± 5.6%) at 30 days on substrate 1 but declined at later stages, while SI performed best on substrate 3 at 30 days (72.3 ± 6.7%) but was less effective after 90 days. The SO and SI mixture showed strong synergistic effects on substrate 1, with peak germination (48.7 ± 5.9%) and seedling formation (45.6 ± 5.1%) at 120 days. Substrates 1 and 3 significantly outperformed 2 (p < 0.05), with 1 promoting rapid early germination and 3 favoring long-term seedling establishment. In contrast, controls without fungi showed less than 5% for all indices, confirming the necessity of symbiotic fungi. Microscopic observations revealed typical orchid mycorrhizal structures and dynamic hyphal turnover, providing histological evidence of the symbiotic mechanism. These findings establish a practical framework for mycorrhizal-assisted propagation and contribute to the ecological cultivation and conservation of D. officinale.
1. Introduction
Orchids, comprising nearly 30,000 species worldwide, represent one of the most diverse flowering plant families [1,2]. As global flagship species, their conservation has long been a major focus for plant biologists [3,4]. However, effective conservation and sustainable utilization of orchids are particularly challenging due to their obligate dependence on complex biotic interactions [5,6]. In particular, mycorrhizal fungi play critical roles throughout the orchid life cycle, from seed germination to maintaining associations in adulthood [7,8].
Mycorrhizal fungi play a pivotal role in regulating plant populations by influencing seedling establishment and species coexistence [9]. Orchids typically produce a vast number of dust-like seeds per fruit and are entirely dependent on specific mycorrhizal fungi for germination and subsequent seedling development [10,11]. The application of orchid mycorrhizal fungi (OMFs) has been proposed as an effective strategy for seed-based orchid conservation [12,13].
During symbiotic germination, compatible OMFs can rapidly and efficiently promote seed germination and seedling development, whereas non-compatible fungi may induce germination but fail to sustain further growth [14,15,16]. In natural habitats, fungal partners often shift during orchid development from seedling to adult stages, with many studies reporting that OMFs experience a taxonomic and functional bottleneck at the germination stage [17,18,19]. Conversely, other studies have shown that diverse OMF taxa can promote germination and seedling development in vitro, albeit with varying efficiencies, such as Spiranthes australis [20] and Gymnadenia conopsea [21].
Dendrobium officinale is an epiphytic or lithophytic orchid widely distributed in subtropical areas, especially in karst regions, at elevations from 500 to 1600 m in China [22]. As the most popular medicinal plant in Dendrobium, D. officinale has broad bioactivities, including immunomodulatory, antifatigue, antioxidation, digest-promotion, and sialagogue (stimulation of salivary secretion) activities, as well as antihyperglycemic, antihypertensive, hepatoprotective, and antitumor activities [23].
For D. officinale, multiple isolates, including Tulasnella, Sebacina, and Serendipita species, have been demonstrated to enhance seed germination and seedling growth with varying efficiencies [13,24,25,26]. Moreover, the non-orchid-specific fungus Serendipita indica effectively supports germination and seedling development in D. officinale and other orchids [21,27]. However, as these findings are primarily based on in vitro tests, it remains uncertain which fungal partners should be prioritized for practical conservation in the native habitats of D. officinale.
Protected cultivation substantially contributes to meeting market demand for Dendrobium plants [28]. However, this cultivation mode requires substantial investment [29], advanced technologies (including large-scale seedling production, varietal cultivation, and standardized planting) underpinned by aseptic germination [30,31], and involves high risk alongside high reward [28]. Consequently, its high economic investment, technical complexity, and stringent management render it suitable primarily for industrial-scale production rather than small-scale farming [32].
The substrate and the cultivation techniques influence the survival rate during transplantation, subsequent plant growth, and eventual yield. Substrates provide root support for plants grown ex situ [33] and critically influence product quality in orchid cultivation and seedling production [34]. No universal substrate blend exists for epiphytic orchids across diverse environments; optimal compositions vary regionally due to climatic differences and are species-specific even within the same environment [35]. Multiple substrates are applicable, including plant-derived (e.g., sphagnum, coconut fiber, pine bark), mineral (e.g., vermiculite, expanded clay), and synthetic materials (e.g., polystyrene) [36]. However, no single material or mixture is universally effective, necessitating species- and management-specific evaluations [37].
To obtain the most suitable OMFs and substrate for use in conservation practices and imitation of wild cultivation for this conservation-significant medicinal orchid, in this study, we compared the effects of two mycorrhizal fungi on seed germination and seedling development of D. officinale in three substrate mixtures. The aim of this study was to screen out fungi and substrates that can effectively promote seed germination of D. officinale to support conservation and the imitation of wild cultivation for this endangered medicinal orchid.
2. Materials and Methods
2.1. Materials
2.1.1. Seeds
Plants of D. officinale were cultivated in a plantation in Leqing, Zhejiang, China. Mature fruits of D. officinale, resulting from artificial cross-pollination of cultivated plants, were harvested in November 2021 for subsequent experiments. Seeds from all collected fruits were carefully released, then dried and stored at −20 °C in the Orchid Seed Bank of Yunnan University following our previously established method [38]. Prior to use, seeds were removed from the low-temperature seed bank and equilibrated at room temperature for 24 h. Seed viability was assessed using the 2,3,5-triphenyltetrazolium chloride (TTC) staining method, which indicated a viability rate of 97% [39].
2.1.2. Fungal Strains for Symbiotic Cultures
In this study, two mycorrhizal fungal strains were used to compare their effects on seed germination in D. officinale. The sources of origin and related information about the two fungal strains are summarized in Table 1. Of these, Serendipita officinale (SO) was originally isolated from naturally occurring protocorms and adult roots of D. officinale, which were collected from an original habitat of D. officinale at a limestone mountain in Luotian town, Chongqing, China [13,40]. Serendipita indica (SI) was obtained from the Leibniz Institute DSMZ-German Collection of Microorganisms and Cell Cultures, Braunschweig, Germany, and was first isolated from the rhizosphere soil of the woody shrubs Prosopis juliflora (Swartz) DC. and Zizyphus nummularia (Burm. fil.) Wt. & Arn. in the sandy desert soils of Rajasthan, northwest India [41].
Table 1.
The four orchid mycorrhizal fungi used in this study, with their sources of origin and GenBank accession numbers.
2.1.3. Substrate
Nine substrate components were mixed in specific proportions (Table 2), including coconut husk, thick pine bark (9–12 cm), fine pine bark (3–6 cm), peat soil, volcanic rock, Zhijing stone, charcoal, pumice, and Xian soil. The mixtures were packed into polypropylene woven bags with three distinct substrate ratios. After soaking in water for 3 days to achieve saturation, excess water was drained, and the substrates were autoclaved at 121 °C (103 kPa) for 20 min to eliminate microorganisms and pest eggs (e.g., fungus gnats). Sterilized substrates were cooled and transferred to 24-cell plug trays (75 cm × 45 cm × 6 cm; substrate depth: 4 cm) for subsequent experiments.
Table 2.
Substrate formulations for seed germination of Dendrobium officinale.
2.2. Methods
2.2.1. Fungal Powder with Seeds
SO and SI strains were cultured on potato dextrose agar (PDA) medium (25 ± 2 °C, 7 days, darkness). PDA composition: 200 g L−1 potato extract (filtrate of boiled, peeled potatoes), 20 g L−1 dextrose (Xilong Scientific Co., Ltd., Guangzhou, China), and 20 g L−1 agar (SbaseBio Corporation, Tokyo, Japan). When mycelial diameters reached 3–4 cm, mycelial plugs (1 cm3) were aseptically excised using a sterile scalpel and transferred to Erlenmeyer flasks containing potato dextrose broth (PDB). The flasks were incubated in a rotary shaker (ZQZY-CF8) at 28 ± 2 °C and 180 rpm for 10 days, until dense mycelial biomass had formed. Mycelia were collected on sterile and rinsed with sterile distilled water to remove residual dextrose. The cultured mycelia were collected on sterile gauze and rinsed with sterile distilled water to remove residual dextrose. The rinsed mycelia were then mixed with lyophilized agar powder (SbaseBio Corporation, Tokyo, Japan) at a 1:1 (w/w) ratio and ground into a homogeneous powder using a homogenizer. After drying at 28 °C for 4 h, the fungal powder was packed in a valve bag and stored at 4 °C. Three fungal powders were prepared: (i) SO powder, (ii) SI powder, and (iii) a 1:1 (w/w) homogenized blend of SO and SI powders. A 0.03 g aliquot of Dendrobium officinale seeds was mixed with three fungal powder variants: SO, SI, and SO/SI blend (1:1 ratio). The control consisted of agar powder mixed with D. officinale seeds.
2.2.2. Seeding
Seeds mixed with fungal powder were sown on substrates 1–3 at 0.2 g (ca. 30 seeds) per cell in a plug tray, with 15 plug tray replicates per treatment. Plug trays were sealed with polyethylene film and incubated under natural light in a greenhouse (25 ± 5 °C, 60 ± 10% RH).
2.2.3. Data Collection and Statistical Analysis
For each treatment, the number of seeds and the status of seed germination in 32 holes were assessed and recorded at 30, 60, 90, and 120 days after sowing. Seed germination and seedling development were divided into six stages as follows: Stage 0, no germination; Stage 1, embryo swollen and green but still covered with its testa (germination); Stage 2, embryo swollen some more, forming a spherule, seed coat broken and lost (protocorm formation); Stage 3, early protocorm showing a pointed vegetative apex (protocorm differentiation); Stage 4, seedling with emergence of first leaf; and Stage 5, emergence of second leaf and further development [42,43]. We used Stage 0, Stage 1, Stages 2–3, and Stages 4–5 to determine no germination, seed germination, protocorm formation, and seedling development, respectively. The total number of seeds (t), germinated seeds (g), protocorms (p), and seedlings (s) were used to calculate the percentages of germinated seeds (G), protocorms (P), and seedlings (S) as G = (g + p + s)/t, P = (p + s)/t, and S = s/t, respectively.
Statistical analyses, including one-way analysis of variance (ANOVA) and the least significant difference (LSD) post hoc test, were conducted using IBM SPSS Statistics (Version 25). Graphs were generated using Origin 2018 (OriginLab Corporation, Northampton, MA, USA).
2.2.4. Observations on Symbiosis Establishment
To determine whether mycorrhizal symbiosis was successfully established between D. officinale and the fungal isolates SO and SI, protocorms from different treatments (15 samples per treatment) were fixed in FAA at 60 days post-inoculation period. The fixed protocorm samples were vacuumed for 15 min. After dehydration in an ethanol series [70, 85, 95, 100, and 100% (v/v); 1.5 h each step] at room temperature, the samples were infiltrated in 1:2 (v/v) LR (London Resin) white acrylic resins (L9774; Sigma-Aldrich, St. Louis, MO, USA): ethanol for 1–2 h, 2:1 (v/v) LR white acrylic resins: ethanol for 2 h, and 100% LR white acrylic resins overnight at 4 °C, and finally embedded in embedding capsules with LR white acrylic resins. Transverse sections (4 μm thick) were cut from LR White-embedded samples using an ultramicrotome (Leica RM2245, Wetzlar, Germany) [21]. The sections were stained with 1% (w/v) toluidine blue O (TBO) for 10–15 min, briefly rinsed in distilled water, and observed under a light microscope (Leica DM3000 LED, Wetzlar, Germany).
3. Results
3.1. Effectiveness of Fungi on Seed Germination of Dendrobium officinale in Three Substrate Combinations
3.1.1. Substrate 1
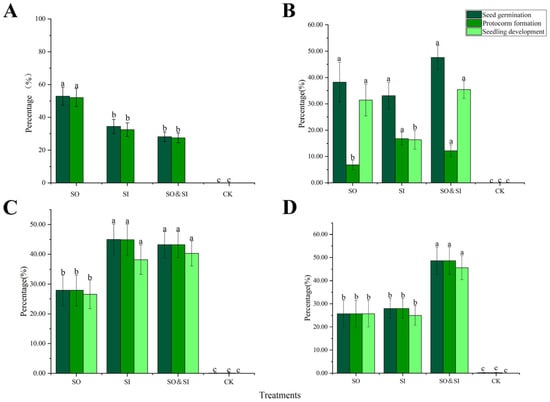
At 30 days after incubation, germination was observed in D. officinale seeds treated with SO, SI, and the SO and SI, whereas no germination occurred in the control. The germination percentage in SO treatment (52.9 ± 5.6%) was significantly higher than in the other three treatments (p < 0.05; Figure 1A). At 60 days, seed germination increased significantly in SO and SI treatment (47.6 ± 4.5%) (Figure 1B), and the control still showed no germination. At 90 days, SI treatment yielded the highest seed germination (45.0 ± 5.2%) among all treatments (Figure 1C), and few seeds germinated in the control (0.1 ± 0.1%). At 120 days, the germination percentage in SO and SI treatment (48.7 ± 5.9%) was significantly higher than in any other treatments (p < 0.05; Figure 1D).
Figure 1.
Seed germination, protocorm formation, and seedling formation of different treatments and time periods of symbiotic seed germination on substrate 1 (hick pine bark/fine pine bark/Xian soil/charcoal/pumice/Zhijing stone/coconut husk = 5:4:1:1:1:1:1). (A–D) at 30, 60, 90, and 120 days after incubation. In each panel, different letters indicate significant differences (p < 0.05). Abbreviation: SO, Serendipita officinale; SI, Serendipita indica; CK: Control check.
3.1.2. Substrate 2
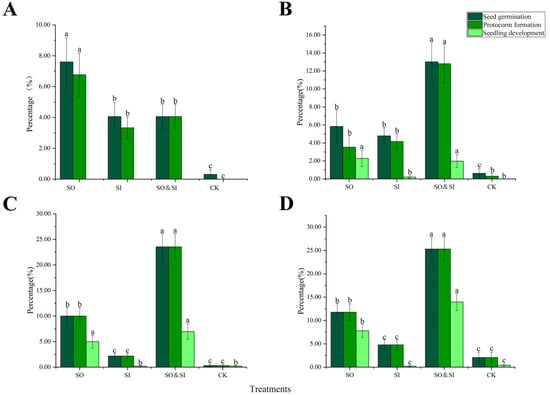
At 30 days after incubation, germination was also observed in D. officinale seeds treated with SO, SI, and the SO and SI, while no germination occurred in the control group (Figure 2A). However, germination percentage was low across the three treatments (7.1 ± 1.6%, 4.1 ± 0.9%, and 4.1 ± 0.8%, p < 0.05). At 60 days after incubation, seed germination had significantly increased in SO and SI treatment (13.2 ± 2.2%) (Figure 2B), and the control group had few germinated seeds (0.6 ± 0.5%). At 90 days after incubation, the seed germination rate of the SO and SI treatments was still rising (23.5 ± 2.5%; Figure 2C). At 120 days after incubation, the percentage of seed germination in SO and SI treatment (25.3 ± 2.5%) was significantly higher than in any other treatment (p < 0.05; Figure 2D).
Figure 2.
Seed germination, protocorm formation, and seedling formation of different treatments and time periods of symbiotic seed germination on substrate 2 (fine pine bark/volcanic rock = 2:1). (A–D) at 30, 60, 90, and 120 days after incubation. In each panel, different letters indicate significant differences (p < 0.05). Abbreviation: SO, Serendipita officinale; SI, Serendipita indica; CK: Control check.
3.1.3. Substrate 3
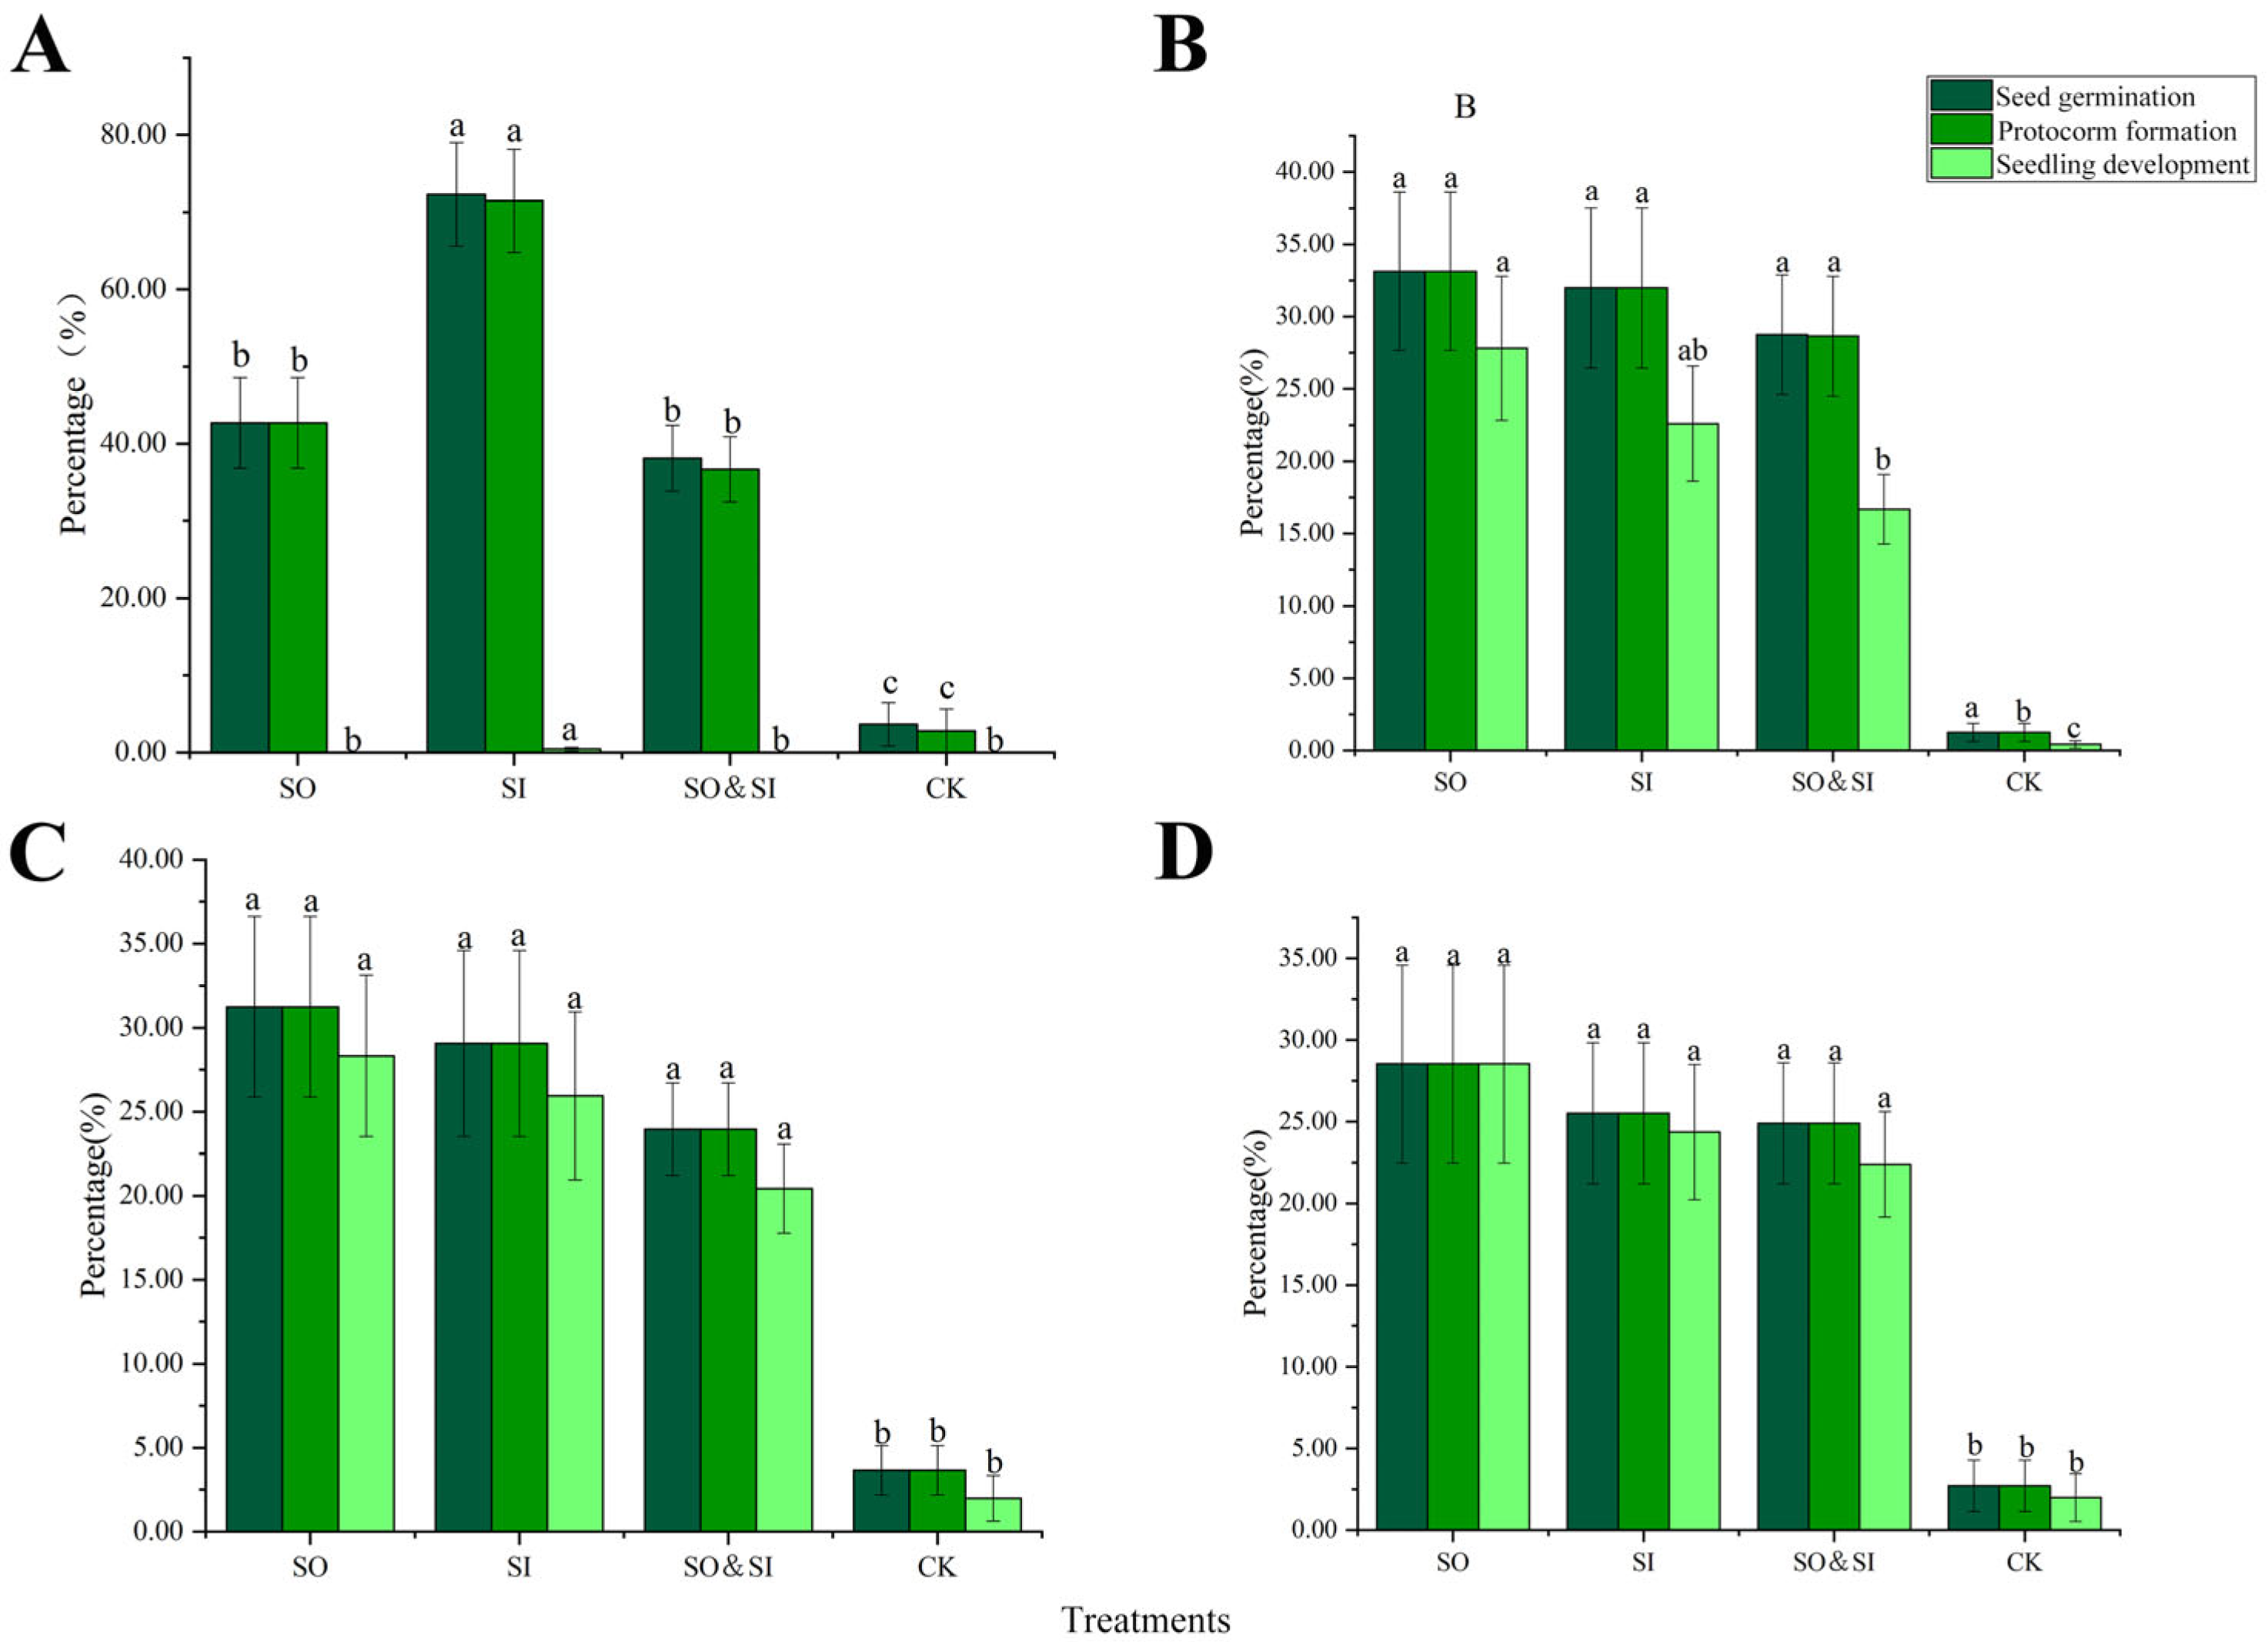
Seed germination of D. officinale occurred across all four treatments by day 30 of incubation. The SI treatment exhibited the highest germination rate (72.3 ± 6.7%) at this stage (Figure 3A). No significant differences in germination were observed among the three fungal treatments at day 60 (all p > 0.05; Figure 3B). However, by day 90, germination in the SI treatment significantly decreased to 22.6 ± 4.0% (Figure 3C). Similarly, the germination rates among the three fungal treatments remained statistically comparable (p > 0.05) at day 120 (Figure 3D).
Figure 3.
Seed germination, protocorm formation, and seedling formation of different treatments and time periods of symbiotic seed germination on substrate 3 (coconut husk/fine pine bark/peat soil = 1:1:1). (A–D) at 30, 60, 90, and 120 days after incubation. In each panel, different letters indicate significant differences (p < 0.05). Abbreviation: SO, Serendipita officinale; SI, Serendipita indica; CK: Control check.
3.2. Effectiveness of Fungi on Protocorm Formation of Dendrobium officinale in Three Substrate Combinations
3.2.1. Substrate 1
At 30 days after incubation, protocorms were observed only in three fungal treatments; no protocorms formed in the control. The protocorm formation percentage in SO treatment (52.1 ± 5.5%) was significantly higher than in SI treatment (32.5 ± 4.2%; p < 0.05) and in SO and SI treatment (27.5 ± 3.0%, p < 0.05) treatments (Figure 1A). At 60 days after incubation, protocorm formation was decreased in SO and SI treatments, but protocorms increased in SO and SI treatments (Figure 1B). At 90 days after incubation, the highest protocorm formation occurred in SI treatment (44.9 ± 5.1%), which was not significantly different from that in SO and SI treatment (43.2 ± 4.4%), but significantly higher than in SO treatments (p < 0.05; Figure 1C). The percentage of protocorm formation in SO and SI treatment (48.7 ± 5.9%) was significantly higher than in any other treatment (p < 0.05) at 120 days after incubation (Figure 1D).
3.2.2. Substrate 2
At 30 days after incubation, protocorms were present in all fungal treatments; however, the percentages were low (6.8 ± 1.4%, 3.3 ± 0.7%, and 4.1 ± 0.8%, p < 0.05; Figure 2A). Protocorm formation had significantly increased in SO and SI treatment (12.8 ± 2.2%) (Figure 2B), and the control group had few protocorms (0.3 ± 0.3%) at 60 days after incubation. At 90 days after incubation, protocorm formation was decreased in SI treatment, but protocorms increased in SO and SO and SI treatments (Figure 2C). At 120 days after incubation, the percentage of protocorm formation in SO and SI treatment (25.3 ± 2.5%) was significantly higher than in any other treatment (p < 0.05; Figure 2D).
3.2.3. Substrate 3
Protocorm formation was observed in all treatments by day 30 of incubation (Figure 3A); the highest protocorm formation occurred in the SI treatment (71.5 ± 6.7%), which was significantly different from that in the other two fungal treatments. No significant differences in protocorm formation were observed among the three fungal treatments at day 60, day 90, and day 120 (all p > 0.05; Figure 3B–D). The percentage of protocorm formation was very close to that of the percentage of seed germination in these stages. The SO treatment exhibited the highest protocorm rate (33.1 ± 5.4%, 31.2 ± 5.4%, 28.5 ± 6.1%) at day 60, day 90, and day 120, respectively (Figure 3B–D).
3.3. Effectiveness of Fungi on Seedling Development of Dendrobium officinale in Three Substrate Combinations
3.3.1. Substrate 1
No seedlings were observed in all treatments at 30 days after incubation (Figure 1A). However, seedlings were observed in three fungal treatments at 60 days after incubation, with the percentages of seedlings increased greatly compared with 30 days ago, respectively (Figure 1B). At this stage, seedling percentages in SO and SI (35.4 ± 3.3%) and SO (31.4 ± 6.1%) treatments were significantly higher than in SI treatments and the control. At 90 days after incubation, the highest seedling formation occurred in SO and SI treatments (40.3 ± 4.2%), which was not significantly different from that in SI treatments (38.2 ± 4.9%), but significantly higher than in SO treatments (p < 0.05; Figure 1C). The percentage of seed germination in SO and SI treatment (45.6 ± 5.1%) was significantly higher than in any other treatments (p < 0.05) at 120 days after incubation (Figure 1D). Notably, no seedlings formed in the control throughout the experiment.
3.3.2. Substrate 2
At 30 days after incubation, no seedlings were found in all treatments (Figure 2A). At 60 days after incubation, a few seedlings were found in SO (2.3 ± 0.9%), SI (0.2 ± 0.1%), and SO and SI (1.98 ± 0.7%) treatments (Figure 2B). At 90 days after incubation, the percentages of seedlings in SO and SI and SO treatments (6.98 ± 1.5% vs. 5.0 ± 1.2%; p > 0.05) were very close and still significantly higher than those in SI treatment and control (Figure 2C). At 120 days after incubation, the percentage of seedlings in SO and SI treatment (14.0 ± 1.8%) was significantly higher than in SO treatment (7.8 ± 1.4%) and SI treatment (0.2 ± 0.1%), respectively (all p < 0.05; Figure 2D). Moreover, the percentage of seedlings in the control was similar to the SI treatment at day 90 and day 120.
3.3.3. Substrate 3
Seedling formation of D. officinale was only found in SI treatments by day 30 of incubation (0.4 ± 0.2%) (Figure 3A). Then, seedlings formed in all treatments at day 60 (p < 0.05). There were no significant differences in the percentages of seedlings between SO treatment (27.8 ± 5.0%) and SI treatment (32.0 ± 5.5%; p > 0.05), and both were significantly higher than that in other treatments (all p < 0.05; Figure 3B). No significant differences in seedling formation were observed among the three fungal treatments at day 90 and day 120 (all p > 0.05; Figure 3C,D). The SI and SO treatments exhibited the highest seedling rate (29.1 ± 5.0%, 28.5 ± 6.1%) at day 90 and day 120, respectively.
3.4. Colonization of Fungi in Protocorm
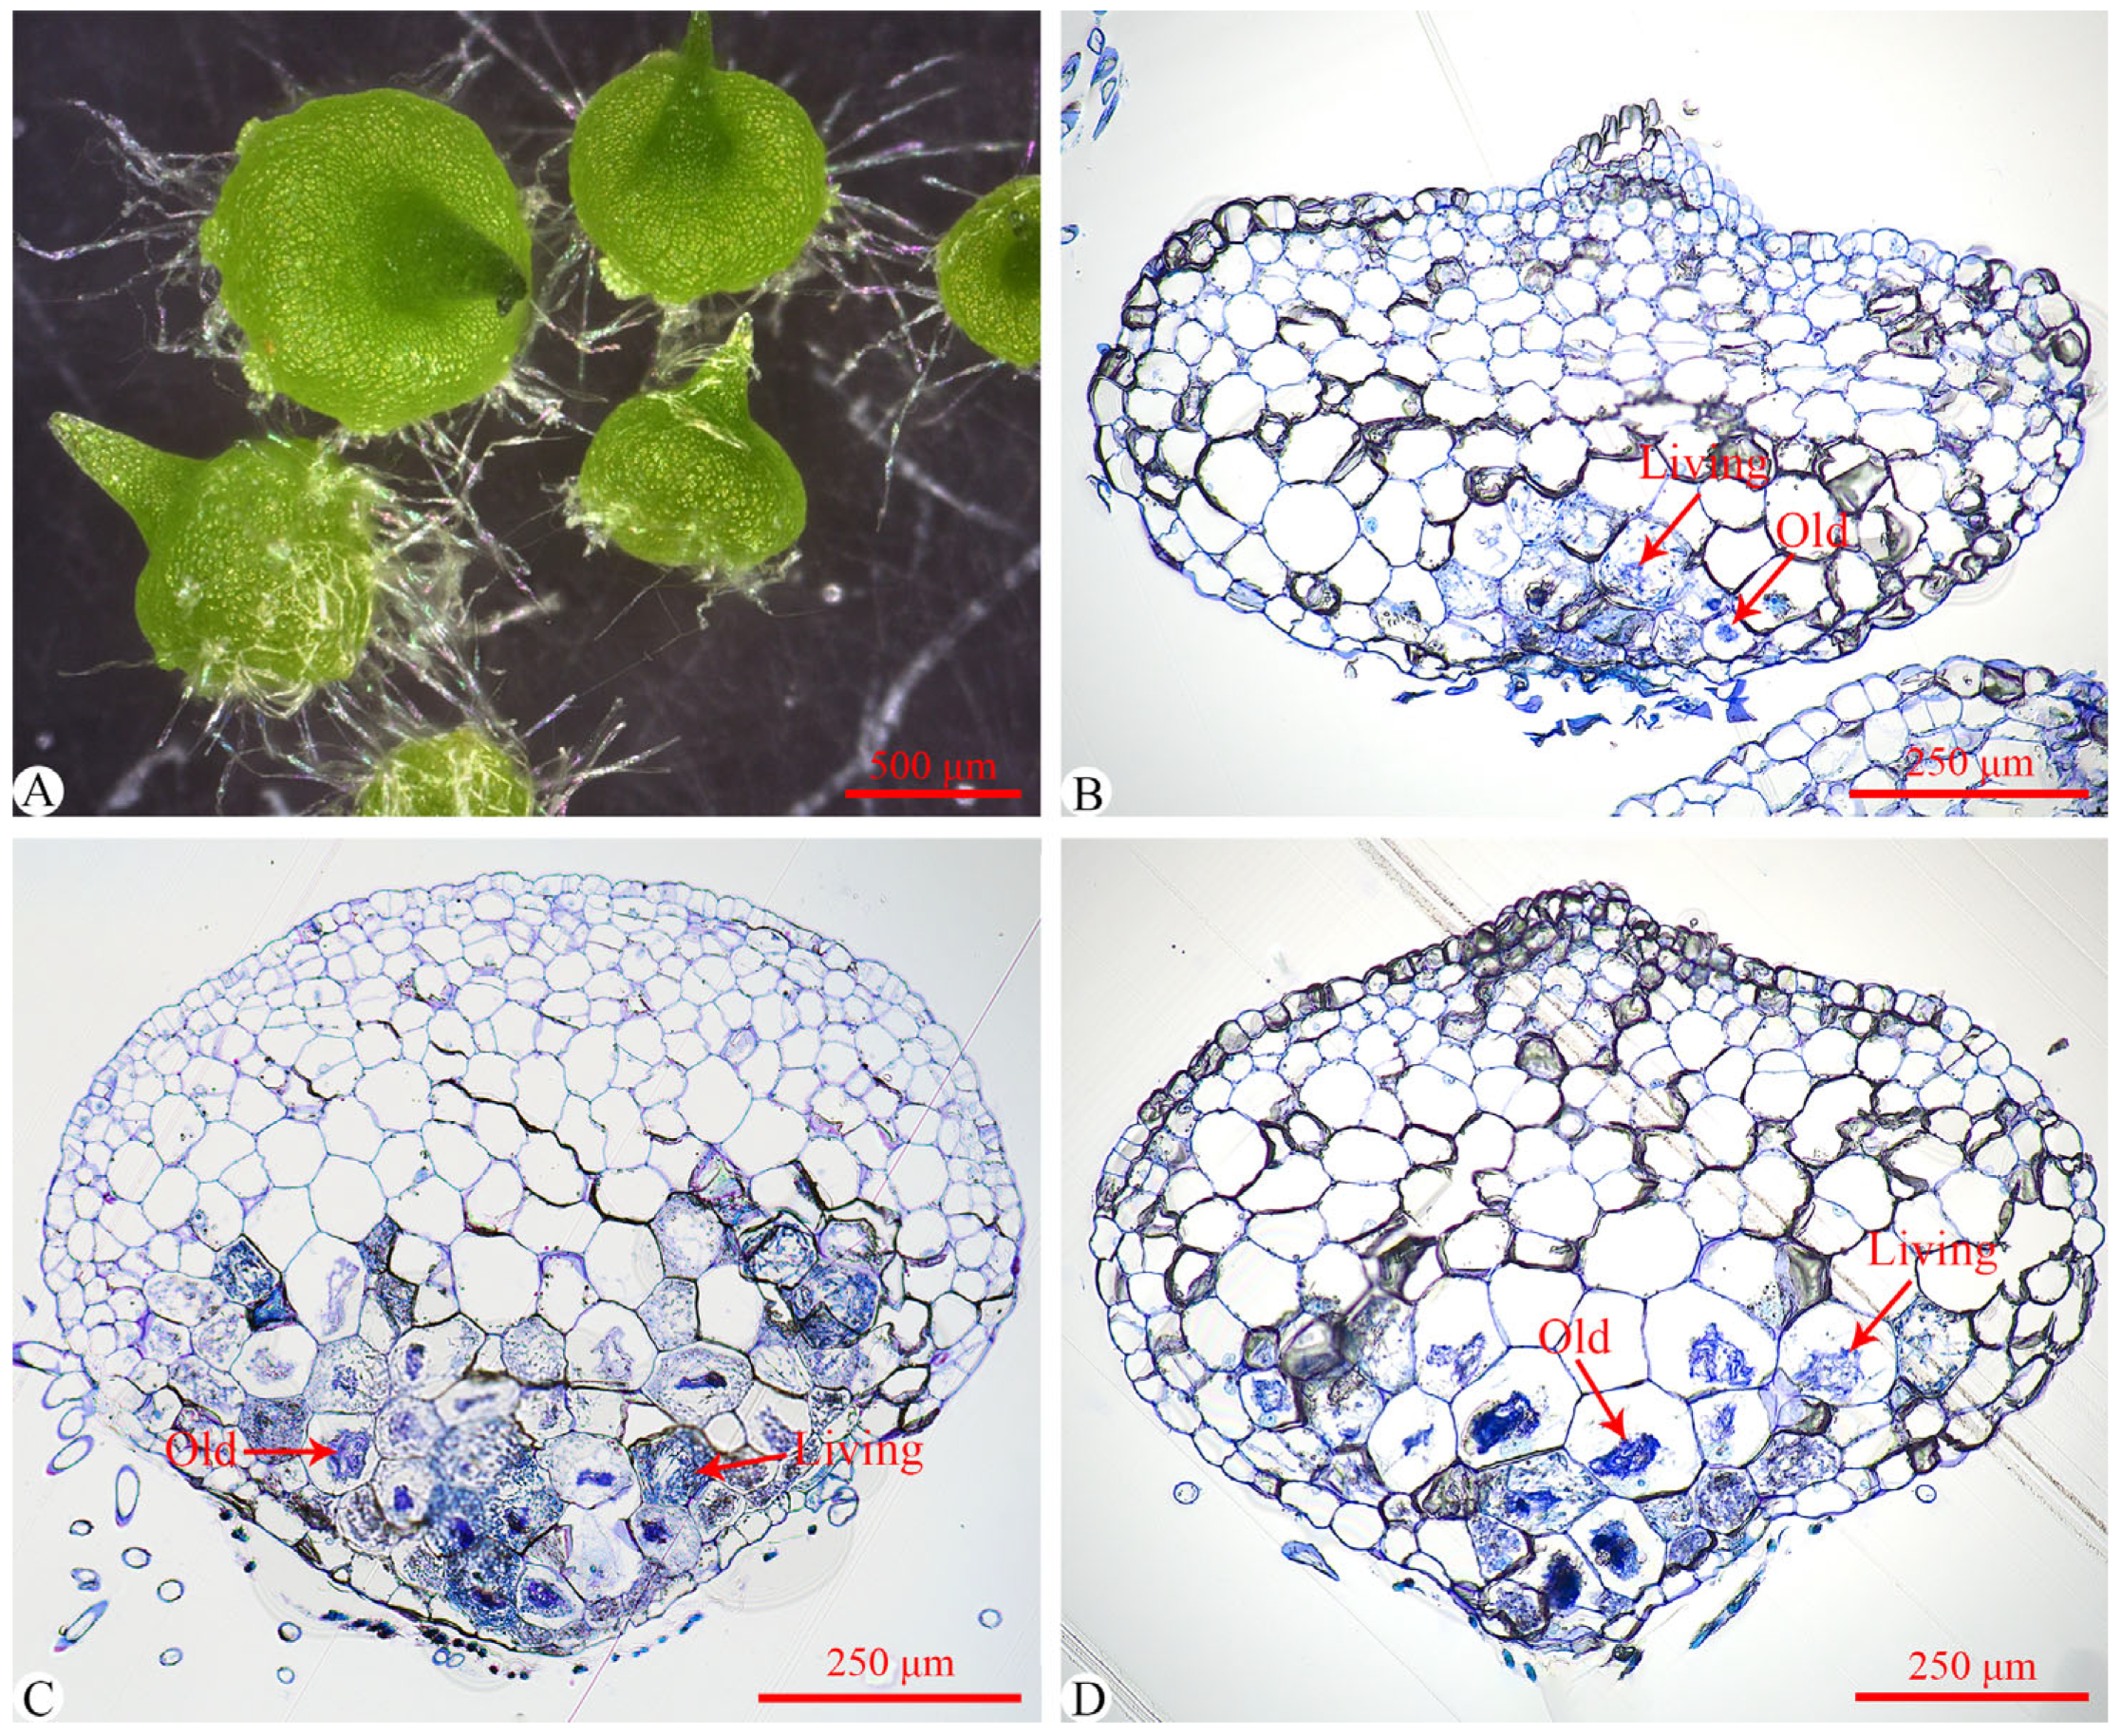
At 60 days post-incubation, abundant clear hyphal coils (pelotons) were observed in all treated protocorms. Intracellular mycelia were localized predominantly in the basal regions of protocorms (Figure 4), which correspond to future root initiation sites. Two peloton types were identified: (i) living pelotons with intact hyphae (Figure 4B–D) and (ii) old pelotons (Figure 4B–D) undergoing terminal degradation (occasionally coexisting within a single cell).
Figure 4.
The colonization of different fungi in Dendrobium officinale protocorms. (A) Protocorms germinated by fungus-seed symbiosis for 60 d at different locations. (B–D) represent the colonization of SI, SO, SO and SI in Dendrobium officinale protocorms, respectively. Red arrows: mycelial clusters.
4. Discussion
This study demonstrates that both substrate composition and fungal compatibility are decisive factors governing the successful symbiotic germination and seedling establishment of D. officinale. Among the tested combinations, substrate 3 (coconut husk/fine pine bark/peat soil = 1:1:1) and the fungal strain Serendipita officinale (SO) exhibited the highest efficiency in promoting germination and sustaining seedling growth. The synergistic interaction between SO and S. indica (SI), particularly on well-aerated substrates, further indicates that complementary fungal functions can enhance nutrient availability and plant vigor. Collectively, these findings provide a strong basis for developing a practical, fungus-assisted propagation system for D. officinale.
As epiphytic orchids, Dendrobium species obtain water and nutrients mainly from atmospheric moisture and organic matter that accumulate around their aerial roots [44]. Therefore, the physical and chemical characteristics of substrates—including aeration, porosity, water- and nutrient-holding capacity, and pH—are critical determinants of seed germination and subsequent growth under cultivation [45,46,47,48]. The results of this study demonstrate that substrate composition has a pronounced effect on the symbiotic germination and seedling development of D. officinale. Since most Dendrobium species are epiphytic and seedling viability is low, the most suitable potting mixture for acclimatization should have good permeability and retain high humidity [49]. The three substrates of this study primarily differed in their air permeability and water-retention capacity, which likely shaped the different germination and growth responses observed. Substrate 1, composed of pine bark, pumice, and coconut husk, promoted rapid germination owing to its excellent aeration and moisture balance [50,51,52,53]. Its moderate water-holding capacity required irrigation only every 7–10 days, which likely supported early and efficient mycorrhizal colonization. However, its relatively low nutrient content may have constrained subsequent seedling growth. Substrate 2, formulated with volcanic rock to assess the drought tolerance of the SI strain, offered excellent aeration but limited water retention, necessitating watering approximately every three days. In contrast, substrate 3 exhibited the highest water-holding capacity but the lowest aeration, thus requiring irrigation only about once per month, providing optimal long-term support for seedling establishment. The combination of porous, moderately acidic organic materials with the nutrient-buffering capacity of peat maintained stable moisture and nutrient availability, thereby creating a favorable microenvironment for sustained mycorrhizal activity [54]. These findings are consistent with previous studies showing that substrate texture and organic content strongly influence orchid root physiology and the establishment of fungal symbioses [55,56,57]. Collectively, these results highlight that appropriate substrate formulation is as crucial as fungal compatibility for successful symbiotic propagation.
The direct sowing technology with symbiotic fungi has been employed in ecological cultivation, and plants grown on substrates mixed with fungi develop stronger root systems, thicker stems, and increased yield [55]. Mycorrhizal technologies can substantially streamline seedling production while enhancing germination, survival, and early growth [58,59]. Each capsule of D. officinale contains thousands of dust-like seeds with an undifferentiated embryo and no endosperm or cotyledon [42]. Consequently, seed germination is strictly dependent on the acquisition of carbon and mineral nutrients from compatible mycorrhizal fungi, and subsequent seedling development also relies on fungal partners to facilitate water and nutrient uptake [60,61]. In recent years, effective symbiotic fungi have been isolated and identified from the roots of several Dendrobium species, including D. officinale, D. nobile, D. chrysotoxum, and D. devonianum, enabling successful symbiotic germination and subsequent growth [24,59,62]. These low-cost, user-friendly approaches make it possible to complete the entire production cycle, from sowing to harvest, under near-natural conditions without reliance on pesticides or synthetic fertilizers [63,64]. Continued refinement of these technologies is expected to further contribute to the sustainable development and large-scale cultivation of the Dendrobium industry.
In orchid symbiotic germination, compatible fungi support both seed germination and seedling development, whereas incompatible fungi may initiate germination but cannot sustain further growth [14,15,16]. A previous study tested three fungal strains, Micorascuo sp. G3, Chaetomium sp. G4, and Mycena osmundicola, isolated from the roots of Liparis nervosa and Dendrobium hancockii, for their effects on D. officinale seed germination [58,59]. Although all strains promoted germination up to protocorm formation (Stage 2 or 3), none supported further development into seedlings [64,65].
Both Serendipita officinale (SO) and S. indica (SI) were identified as compatible mycorrhizal partners of D. officinale [13,27,40], as evidenced by the presence of characteristic pelotons within protocorm cells, confirming active fungal colonization and nutrient exchange (Figure 4B–D). Although both fungal strains facilitated seed germination and subsequent seedling development, their effects differed in both timing and magnitude. SO primarily enhanced early germination, whereas SI supported seedling development over a more extended period. The higher germination and seedling formation observed under the combined SO + SI treatment on substrate 1, significantly exceeding the outcomes of either fungus alone, indicates a potential synergistic interaction between the two strains. This synergy suggests that complementary functional roles among compatible fungi may enhance overall symbiotic efficiency during orchid early development. This temporal complementarity suggests that different Serendipita species may specialize in distinct developmental phases, a phenomenon also reported in other Dendrobium species [27,66]. With respect to early developmental dynamics, accumulating evidence indicates that orchids may associate with different fungal partners at successive ontogenetic stages. Only a subset of the fungi capable of initiating germination appears able to sustain subsequent development under natural conditions [17,18]. A similar pattern has been observed in ex situ systems, where a broader range of fungal isolates can promote the earliest stages of seed germination, whereas fewer taxa support continued seedling growth [15]. Collectively, these findings support the presence of an “hourglass” or bottleneck pattern in mycorrhizal symbiont diversity throughout orchid development, characterized by the highest degree of fungal specificity at the advanced seedling stage. The presence of characteristic pelotons in protocorms under all treatments verified successful intracellular colonization and nutrient exchange [16,67]. The superior performance of the SO–substrate 3 combination underscores the importance of integrating compatible fungal symbionts with substrates of appropriate physical and chemical characteristics to maximize germination efficiency and promote seedling formation.
Notably, in treatments combining the SO strain with the three substrates, both seed germination rates and protocorm formation after 60 days were lower than those recorded at 30 days. Orchid seed germination and early development progress through six stages, and only a portion of seeds successfully advance to protocorm formation and subsequent seedling growth. Seed viability itself changes dynamically from pollination to maturity, as the seed coat progressively hardens, and its permeability decreases, leading to reduced germination percentages [68]. Furthermore, the physical properties of the substrates likely contributed to the temporal decline observed. Compaction is known to inhibit germination and early growth by reducing soil aeration and lowering soil temperature [69]. Because substrate compaction greatly decreases porosity and thereby restricts gas diffusion [70], it can impose a significant barrier to oxygen availability—one of the most limiting factors influencing orchid seed germination. Although the precise mechanisms by which restricted gas exchange suppresses germination remain to be fully clarified.
This study demonstrates that integrating optimized Serendipita symbionts with suitable substrate formulations provides an efficient, cost-effective, and scalable strategy for the propagation of D. officinale. The fungus-assisted direct-seeding system established here significantly enhances germination and post-transplant survival while preserving the natural mycorrhizal association essential for ecological adaptation. Compared with conventional tissue culture, this symbiotic approach reduces reliance on sterile facilities and synthetic media, offering a sustainable alternative for ex situ conservation and semi-natural cultivation. This integrative strategy also provides a valuable model for developing symbiotic propagation systems in other endangered or economically important orchids with similar mycorrhizal requirements.
5. Conclusions
This study established a symbiotic seedling cultivation system for D. officinale by combining a two-stage “seed germination–seedling development” strategy with synergistic fungal strains and substrate selection, thereby achieving full-cycle optimization from seed to seedling. The combination of symbiotic fungus SO and substrate 3 achieved stable seed germination and seedling formation at later stages compared with the other treatments (p < 0.05). The high porosity, together with the adequate water-holding capacity of substrate 3, along with the mycelial network, created a hypoxic environment that effectively supported seed germination and early seedling development, thus overcoming the technical bottleneck of traditional tissue culture, which relies heavily on aseptic facilities.
Author Contributions
N.L.: Methodology, Writing—original draft; K.T.: Writing—review and editing; J.Y.: Resources; J.S.: Resources; J.G.: Conceptualization, Funding acquisition, Investigation, Methodology, Project administration, Supervision, Writing—review and editing; H.H.: Writing—review and editing, Project administration, Supervision. All authors have read and agreed to the published version of the manuscript.
Funding
This work was supported by the Innovation Guidance and Technology-Based Enterprise Cultivation Program Project of the Yunnan Provincial Department of Science and Technology (202304BP090006).
Data Availability Statement
The original contributions presented in this study are included in the article. Further inquiries can be directed to the corresponding authors.
Acknowledgments
We thank Xinju Wang from Yunnan Normal University for helping with manuscript revisions, Lei Tao from Yunnan University for helping with data analysis, and Bofeng Song from the University of Western Australia for helping with manuscript revisions and data analysis.
Conflicts of Interest
The authors declare no conflicts of interest. The funders had no role in the design of the study; in the collection, analyses, or interpretation of data; in the writing of the manuscript; or in the decision to publish the results. Authors Jian Yue and Juan Su were employed by the company Guangnan Yaowanggu Biological Technology Company Limited, Wenshan, 663300, China. The remaining authors declare the absence of any commercial or financial relationships that could be construed as a potential conflict of interest.
References
- Chase, M.W.; Cameron, K.M.; Freudenstein, J.V.; Pridgeon, A.M.; Salazar, G.; van den Berg, C.; Schuiteman, A. An Updated Classification of Orchidaceae. Bot. J. Linn. Soc. 2015, 177, 151–174. [Google Scholar] [CrossRef] [Scilit]
- Pérez-Escobar, O.A.; Bogarín, D.; Przelomska, N.A.S.; Ackerman, J.D.; Balbuena, J.A.; Bellot, S.; Bühlmann, R.P.; Cabrera, B.; Cano, J.A.; Charitonidou, M.; et al. The Origin and Speciation of Orchids. New Phytol. 2024, 242, 700–716. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- IUCN. 2004 IUCN Red List of Threatened Species: A Global Species Assessment; Baillie, J.E.M., Hilton-Taylor, C., Stuart, S.N., Eds.; IUCN: Gland, Switzerland; Cambridge, UK, 2004; ISBN 2-8317-0826-5. [Google Scholar]
- Swarts, N.D.; Dixon, K.W. Terrestrial Orchid Conservation in the Age of Extinction. Ann. Bot. 2009, 104, 543–556. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fay, M.F. Orchid Conservation: How Can We Meet the Challenges in the Twenty-First Century? Bot. Stud. 2018, 59, 16. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, H.; Liu, Z.; Jin, X.; Gao, J.; Chen, Y.; Liu, Q.; Zhang, D.-Y. Assessing Conservation Efforts against Threats to Wild Orchids in China. Biol. Conserv. 2020, 243, 108484. [Google Scholar] [CrossRef] [Scilit]
- Cameron, D.D.; Leake, J.R.; Read, D.J. Mutualistic Mycorrhiza in Orchids: Evidence from Plant–Fungus Carbon and Nitrogen Transfers in the Green-Leaved Terrestrial Orchid Goodyera repens. New Phytol. 2006, 171, 405–416. [Google Scholar] [CrossRef] [Scilit]
- Li, T.; Yang, W.; Wu, S.; Selosse, M.-A.; Gao, J. Progress and Prospects of Mycorrhizal Fungal Diversity in Orchids. Front. Plant Sci. 2021, 12, 646325. [Google Scholar] [CrossRef] [Scilit]
- Tedersoo, L.; Bahram, M.; Zobel, M. How Mycorrhizal Associations Drive Plant Population and Community Biology. Science 2020, 367, eaba1223. [Google Scholar] [CrossRef] [Scilit]
- Arditti, J.; Ghani, A.K.A. Numerical and Physical Properties of Orchid Seeds and Their Biological Implications. New Phytol. 2000, 145, 367–421. [Google Scholar] [CrossRef] [Scilit]
- Dearnaley, J.; Perotto, S.; Selosse, M.-A. Structure and Development of Orchid Mycorrhizas. In Molecular Mycorrhizal Symbiosis; John Wiley & Sons, Ltd.: Hoboken, NJ, USA, 2016; pp. 63–86. ISBN 978-1-118-95144-6. [Google Scholar]
- Batty, A.L.; Brundrett, M.; Dixon, K.W.; Sivasithamparam, K. In Situ Symbiotic Seed Germination and Propagation of Terrestrial Orchid Seedlings for Establishment at Field Sites. Aust. J. Bot. 2006, 54, 375–381. [Google Scholar] [CrossRef] [Scilit]
- Wang, X.-J.; Wu, Y.-H.; Ming, X.-J.; Wang, G.; Gao, J.-Y. Isolating Ecological-Specific Fungi and Creating Fungus-Seed Bags for Epiphytic Orchid Conservation. Glob. Ecol. Conserv. 2021, 28, e01714. [Google Scholar] [CrossRef] [Scilit]
- Swarts, N.D.; Sinclair, E.A.; Francis, A.; Dixon, K.W. Ecological Specialization in Mycorrhizal Symbiosis Leads to Rarity in an Endangered Orchid. Mol. Ecol. 2010, 19, 3226–3242. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Rasmussen, H.N.; Dixon, K.W.; Jersáková, J.; Těšitelová, T. Germination and Seedling Establishment in Orchids: A Complex of Requirements. Ann. Bot. 2015, 116, 391–402. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Rafter, M.; Yokoya, K.; Schofield, E.J.; Zettler, L.W.; Sarasan, V. Non-Specific Symbiotic Germination of Cynorkis purpurea (Thouars) Kraezl., a Habitat-Specific Terrestrial Orchid from the Central Highlands of Madagascar. Mycorrhiza 2016, 26, 541–552. [Google Scholar] [CrossRef] [Scilit]
- Bidartondo, M.I.; Read, D.J. Fungal Specificity Bottlenecks during Orchid Germination and Development. Mol. Ecol. 2008, 17, 3707–3716. [Google Scholar] [CrossRef] [Scilit]
- De Long, J.R.; Swarts, N.D.; Dixon, K.W.; Egerton-Warburton, L.M. Mycorrhizal Preference Promotes Habitat Invasion by a Native Australian Orchid: Microtis media. Ann. Bot. 2013, 111, 409–418. [Google Scholar] [CrossRef] [Scilit]
- Givnish, T.J.; Spalink, D.; Ames, M.; Lyon, S.P.; Hunter, S.J.; Zuluaga, A.; Iles, W.J.D.; Clements, M.A.; Arroyo, M.T.K.; Leebens-Mack, J.; et al. Orchid Phylogenomics and Multiple Drivers of Their Extraordinary Diversification. Proc. R. Soc. B Biol. Sci. 2015, 282, 20151553. [Google Scholar] [CrossRef] [Scilit]
- Fuji, M.; Miura, C.; Yamamoto, T.; Komiyama, S.; Suetsugu, K.; Yagame, T.; Yamato, M.; Kaminaka, H. Relative Effectiveness of Tulasnella Fungal Strains in Orchid Mycorrhizal Symbioses between Germination and Subsequent Seedling Growth. Symbiosis 2020, 81, 53–63. [Google Scholar] [CrossRef] [Scilit]
- Gao, Y.; Zhao, Z.; Li, J.; Liu, N.; Jacquemyn, H.; Guo, S.; Xing, X. Do Fungal Associates of Co-Occurring Orchids Promote Seed Germination of the Widespread Orchid Species Gymnadenia conopsea? Mycorrhiza 2020, 30, 221–228. [Google Scholar] [CrossRef] [Scilit]
- Zhu, G.-H.; Ji, Z.-H.; Wood, J.J.; Wood, H.P. Dendrobium. In Flora of China: Orchidaceae; Science Press: Beijing, China, 2009; Volume 25, pp. 367–397. [Google Scholar]
- Lv, G.-Y.; Yan, M.-Q.; Chen, S.-H. Review of Pharmacological Activities of Dendrobium officinale Based on Traditional Functions. China J. Chin. Mater. Medica 2013, 38, 489–493. [Google Scholar] [CrossRef] [Scilit]
- Chen, J.; Wang, H.; Guo, S.-X. Isolation and Identification of Endophytic and Mycorrhizal Fungi from Seeds and Roots of Dendrobium (Orchidaceae). Mycorrhiza 2012, 22, 297–307. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tan, X.M.; Wang, C.L.; Chen, X.M.; Zhou, Y.Q.; Wang, Y.Q.; Luo, A.X.; Liu, Z.H.; Guo, S.X. In Vitro Seed Germination and Seedling Growth of an Endangered Epiphytic Orchid, Dendrobium officinale, Endemic to China Using Mycorrhizal Fungi (Tulasnella sp.). Sci. Hortic. 2014, 165, 62–68. [Google Scholar] [CrossRef] [Scilit]
- Zhang, Y.; Li, Y.-Y.; Chen, X.-M.; Guo, S.-X.; Lee, Y.-I. Effect of Different Mycobionts on Symbiotic Germination and Seedling Growth of Dendrobium officinale, an Important Medicinal Orchid. Bot. Stud. 2020, 61, 2. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xu, Z.-X.; Zhu, X.-M.; Yin, H.; Li, B.; Chen, X.-J.; Fan, X.-L.; Li, N.-Q.; Selosse, M.-A.; Gao, J.-Y.; Han, J.-J. Symbiosis between Dendrobium catenatum Protocorms and Serendipita indica Involves the Plant Hypoxia Response Pathway. Plant Physiol. 2023, 192, 2554–2568. [Google Scholar] [CrossRef] [Scilit]
- Si, J.-P.; Wang, Q.; Liu, Z.-J.; Liu, J.-J.; Luo, Y.-B. Breakthrough in Key Science and Technologies in Dendrobium catenatum Industry. China J. Chin. Mater. Medica 2017, 42, 2223–2227. [Google Scholar] [CrossRef]
- Sugapriya, S.; Mathad, J.C.; Patil, A.A.; Hegde, R.V.; Lingaraju, S.; Biradar, M.S. Evaluation of Dendrobium Orchids for Growth and Yield Grown under Greenhouse. Karnataka J. Agric. Sci. 2012, 25, 104–107. [Google Scholar]
- Vasudevan, R.; van Staden, J. Fruit Harvesting Time and Corresponding Morphological Changes of Seed Integuments Influence in Vitro Seed Germination of Dendrobium nobile Lindl. Plant Growth Regul. 2010, 60, 237–246. [Google Scholar] [CrossRef] [Scilit]
- Naik, S.K.; Bharathi, U. Production Technology of Dendrobium Cultivation; ICAR Research Complex for Eastern Region: Ranchi, India, 2012. [Google Scholar]
- Wu, Y.-Q.; Si, J.-P. Present Status and Sustainable Development of Dendrobium officinale Industry. China J. Chin. Mater. Medica 2010, 35, 2033–2037. [Google Scholar] [CrossRef] [Scilit]
- Kämpf, A.N. Produção Comercial de Plantas Ornamentais; Agropecuária: Guaíba, Brazil, 2000. [Google Scholar]
- de Assis, A.M.; Unemoto, L.K.; Yamamoto, L.Y.; Lone, A.B.; de Souza, G.R.B.; de Faria, R.T.; Roberto, S.R.; Takahashi, L.S.A. Cultivo de orquídea em substratos à base de casca de café. Bragantia 2011, 70, 544–549. [Google Scholar] [CrossRef] [Scilit]
- Shiraki, J.N.; Diaz, E.M. Orquídeas; Secretaria do Verde e do Meio Ambiente: São Paulo, Brazil, 2012. [Google Scholar]
- Dematté, J.B.I.; Dematté, M.E.S.P. Estudos hídricos com substratos vegetais para cultivo de orquídeas epífitas. Pesqui. Agropecuária Bras. 1996, 31, 803–813. [Google Scholar] [CrossRef]
- Berjón, M.A. Los Sustratos Hortícolas y Las Técnicas de Cultivo Sin Suelo. In Proceedings of the la Horticultura Española en la CE; SECH (Sociedad Española de Ciencias Hortícolas): Córdoba, Spain, 1991; pp. 270–280. [Google Scholar]
- Gao, J.-Y.; Liu, Q.; Yu, D.-L. Orchids in Xishuangbanna: Diversity and Conservation; China Forestry Publishing House: Beijing, China, 2014. [Google Scholar]
- Vujanovic, V.; St-Arnaud, M.; Barabé, D.; Thibeault, G. Viability Testing of Orchid Seed and the Promotion of Colouration and Germination. Ann. Bot. 2000, 86, 79–86. [Google Scholar] [CrossRef] [Scilit]
- Wang, X.-J.; Gao, J.-Y.; Li, N.-Q. Serendipita officinale sp. Nov. (Serendipitaceae): A New Species of Orchid Mycorrhizal Fungus. Phytotaxa 2023, 630, 229–240. [Google Scholar] [CrossRef] [Scilit]
- Verma, S.; Varma, A.; Rexer, K.-H.; Hassel, A.; Kost, G.; Sarbhoy, A.; Bisen, P.; Bütehorn, B.; Franken, P. Piriformospora indica, Gen. et Sp. Nov., a New Root-Colonizing Fungus. Mycologia 1998, 90, 896–903. [Google Scholar] [CrossRef] [Scilit]
- Arditti, J. Factors Affecting the Germination of Orchid Seeds. Bot. Rev. 1967, 33, 1–97. [Google Scholar] [CrossRef] [Scilit]
- Stewart, S.L.; Zettler, L.W. Symbiotic Germination of Three Semi-Aquatic Rein Orchids (Habenaria repens, H. quinquiseta, H. macroceratitis) from Florida. Aquat. Bot. 2002, 72, 25–35. [Google Scholar] [CrossRef] [Scilit]
- Atwell, B.J.; Kriedemann, P.E.; Turnbull, C.G.N.; Eamus, D.; Bieleski, R.L. (Eds.) Plants in Action: Adaptation in Nature, Performance in Cultivation; Macmillan Education AU: Melbourne, Australia, 1999. [Google Scholar]
- de Oliveira, L.F.C.; Martinez, M.A.; Pruski, F.F.; Griebeler, N.P.; de Oliveira, G.C. Rotina computacional para a determinação da velocidade de sedimentação das partículas do solo em suspensão no escoamento superficial. Eng. Agríc. 2005, 25, 126–136. [Google Scholar] [CrossRef] [Scilit]
- da Silva, F.F.; Wallach, R.; Chen, Y. Hydraulic Properties of Sphagnum Peat Moss and Tuff (Scoria) and Their Potential Effects on Water Availability. Plant Soil. 1993, 154, 119–126. [Google Scholar] [CrossRef] [Scilit]
- Spomer, L.A.; Berry, W.L.; Tibbitts, T.W. Plant Culture in Solid Media. In Plant Growth Chamber Handbook; Iowa Agricultural and Home Economics Experiment Station: Ames, IA, USA, 1997; pp. 105–118. [Google Scholar]
- Benedetto, A.D. Alternative Substrates for Potted Ornamental Plants Based on Argentinean Peat and Argentinean River Waste: A Review. Floric. Ornam. Biotechnol. 2007, 7, 90–101. [Google Scholar] [CrossRef] [Scilit]
- Zheng, Z.-X. Study on Technique for Propagation and Planting of Several Officinal Dendrobium; Chinese Academy of Forestry: Beijing, China, 2006. [Google Scholar]
- Takane, R.J.; Yanagisawa, S.S.; Góis, E.d.A. Técnicas em Substratos para a Floricultura; Expressão Gráfica e Editora: Fortaleza, Brazil, 2013. [Google Scholar]
- Zandoná, A.P.; de Faria, R.T.; Lone, A.B.; Hoshino, R.T. Substratos alternativos ao esfagno na aclimatização de plântulas de Arundina graminifolia “alba” (Orchidaceae). Ornam. Hortic. 2014, 20, 7–12. [Google Scholar] [CrossRef] [Scilit]
- Mora, M.M.; Assis, A.M.D.; Yamamoto, L.Y.; Pivetta, K.F.L.; Faria, R.T. Resíduos agrícolas e argila expandida no cultivo da orquídea Oncidium baueri Lindl. Semina Ciênc. Agrár. 2015, 36, 39. [Google Scholar] [CrossRef] [Scilit]
- Xue, H.-J.; Shen, X.-D.; Zou, C.-X.; Dong, W. Research Progress of Pumice and Pumice Lightweight Aggregate Concrete Materials. Bull. Chin. Ceram. Soc. 2016, 35, 1536–1540+1546. [Google Scholar] [CrossRef]
- Zanetti, M.; Cazetta, J.O.; de Mattos Júnior, D.; de Carvalho, S.A. Uso de subprodutos de carvão vegetal na formação do porta-enxerto limoeiro “Cravo” em ambiente protegido. Rev. Bras. Frutic. 2003, 25, 508–512. [Google Scholar] [CrossRef] [Scilit]
- Pant, B.; Thapa, D. In Vitro Mass Propagation of an Epiphytic Orchid, Dendrobium primulinum Lindl. through Shoot Tip Culture. Afr. J. Biotechnol. 2012, 11, 9970–9974. [Google Scholar] [CrossRef] [Scilit]
- Han, X.-H.; Sun, J.-L.; Duan, C.-H. Rooting Medium Optimization and Transplanting Matrix Selection of Dendrobium candidum. Guangdong Agric. Sci. 2013, 40, 16–18+23. [Google Scholar] [CrossRef]
- Teixeira Da Silva, J.A.; Hossain, M.M.; Sharma, M.; Dobránszki, J.; Cardoso, J.C.; Zeng, S. Acclimatization of in Vitro-Derived Dendrobium. Hortic. Plant J. 2017, 3, 110–124. [Google Scholar] [CrossRef] [Scilit]
- Tan, X. The Optimization of Planting Main Technical Links in the Production of Dendrobium officinale and Analysis the Content of Some Important Functional Components. Master’s Thesis, Hainan University, Haikou, China, 2014. [Google Scholar]
- Teixeira da Silva, J.A.; Tsavkelova, E.A.; Zeng, S.; Ng, T.B.; Parthibhan, S.; Dobránszki, J.; Cardoso, J.C.; Rao, M.V. Symbiotic in Vitro Seed Propagation of Dendrobium: Fungal and Bacterial Partners and Their Influence on Plant Growth and Development. Planta 2015, 242, 1–22. [Google Scholar] [CrossRef] [Scilit]
- Smith, S.E.; Read, D.J. Mycorrhizal Symbiosis, 3rd ed.; Academic Press: Cambridge, MA, USA; Elsevier: Amsterdam, The Netherlands, 2008. [Google Scholar]
- Shimura, H.; Sadamoto, M.; Matsuura, M.; Kawahara, T.; Naito, S.; Koda, Y. Characterization of Mycorrhizal Fungi Isolated from the Threatened Cypripedium macranthos in a Northern Island of Japan: Two Phylogenetically Distinct Fungi Associated with the Orchid. Mycorrhiza 2009, 19, 525–534. [Google Scholar] [CrossRef] [Scilit]
- Yu, J.; Zhou, X.-F.; Yang, S.-J.; Liu, W.-H.; Hu, X.-F. Design and Application of Specific 16S rDNA-Targeted Primers for Assessing Endophytic Diversity in Dendrobium officinale Using Nested PCR-DGGE. Appl. Microbiol. Biotechnol. 2013, 97, 9825–9836. [Google Scholar] [CrossRef] [Scilit]
- Dan, Y.; Meng, Z.-X.; Guo, S.-X. Effects of Forty Strains of Orchidaceae Mycorrhizal Fungi on Growth of Protocorms and Plantlets of Dendrobium candidum and D. nobile. Afr. J. Microbiol. Res. 2012, 6, 34–39. [Google Scholar] [CrossRef] [Scilit]
- Zhang, L.; Chen, J.; Lv, Y.; Gao, C.; Guo, S. Mycena sp., a Mycorrhizal Fungus of the Orchid Dendrobium Officinale. Mycol. Prog. 2012, 11, 395–401. [Google Scholar] [CrossRef] [Scilit]
- Guo, S.-X.; Xu, J.-T. Isolation and Culture of Fungi Promoting Seed Germination of Shihu Etc Medicinal Plants of Orchid Family (Orchidaceae). Chin. Tradit. Herb. Drugs 1990, 21, 30–31+47. [Google Scholar]
- Zhang, Y.; Wang, S.-W.; Li, N.-Q.; Jin, Q.; Anbazhakan, R.; Dai, Y.-F.; Xiang, Z.-X.; Gao, J.-Y. Ecological Specificity of Fungi on Seedling Establishment in Dendrobium huoshanense: A Narrow Distributed Medicinal Orchid. Mycorrhiza 2025, 35, 41. [Google Scholar] [CrossRef] [Scilit]
- Peterson, R.L.; Massicotte, H.B.; Melville, L.H. Mycorrhizas: Anatomy and Cell Biology; NRC Research Press: Ottawa, ON, Canada; CABI Pub: Wallingford, UK, 2004; ISBN 978-0-660-19087-7. [Google Scholar]
- Dowling, N.; Jusaitis, M. Asymbiotic in Vitro Germination and Seed Quality Assessment of Australian Terrestrial Orchids. Aust. J. Bot. 2012, 60, 592–601. [Google Scholar] [CrossRef] [Scilit]
- Soane, B.D.; Blackwell, P.S.; Dickson, J.W.; Painter, D.J. Compaction by Agricultural Vehicles: A Review I. Soil and Wheel Characteristics. Soil Tillage Res. 1980, 1, 207–237. [Google Scholar] [CrossRef] [Scilit]
- Moldrup, P.; Olesen, T.; Yoshikawa, S.; Komatsu, T.; Rolston, D.E. Three-Porosity Model for Predicting the Gas Diffusion Coefficient in Undisturbed Soil. Soil Sci. Soc. Am. J. 2004, 68, 750–759. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2025 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).