


Abstract
In this paper, we investigate the asymptotic behavior of solutions to a diffusive forest kinematic model, which describes the interactions among young trees, old trees, and airborne seeds. Our study focuses on the stability of the positive equilibrium, the occurrence of Hopf bifurcation yielding spatially homogeneous periodic solutions, and the subsequent Turing instability induced by diffusion in these periodic states. The analysis highlights that the juvenile tree mortality rate, represented by a quadratic function of mature tree density, plays a central dynamical role. Specifically, the parameter corresponding to the mature tree density at which juvenile mortality is minimized serves as a key Hopf bifurcation parameter. This indicates that the system’s transition to periodic solutions and later to diffusion-driven pattern formation can be effectively regulated through this parameter. From an ecological perspective, these results suggest that forest management strategies capable of indirectly influencing factors related to this critical parameter could help control the emergence of spatial patterns, such as forest patches. Furthermore, the functional form of the mortality rate offers a useful foundation for future studies examining how different assumptions regarding tree interaction morphology may influence ecosystem patterning.
Keywords:
forest kinematic model; reaction–diffusion system; Hopf bifurcation; Turing instability of periodic solutions; mortality rate function; pattern formation MSC:
34C23; 34C28; 39B42; 65L07; 65L15
1. Introduction
Forest ecosystems exhibit complex spatiotemporal dynamics arising from the interplay between biological interactions and environmental constraints. Understanding these dynamics is crucial for predicting forest responses to anthropogenic changes and informing conservation strategies. The forest kinematic model, a reaction–diffusion system describing the interactions between young trees , old trees , and airborne seeds , has emerged as a valuable theoretical framework for studying such phenomena [1].
Originally proposed by Kuznetsov et al. [1], this model captures essential ecological processes including growth, mortality, seed dispersal, and notably, a nonlinear, density-dependent mortality rate for young trees, . It is assumed that there exists some optimal value of “old” tree density under which the recruitment of “young” trees is maximal. Considering the qualitative nature of the model, which is often formulated as a quadratic function, with positive a, b, c [2,3]. This specific functional form implies that the mortality of young trees is minimized at a specific old tree density b, introducing a critical nonlinearity that can profoundly influence the system’s dynamics. Recent modeling work has demonstrated that such internal nonlinearities are key to understanding forest resilience under external stress. Satoru Iwasaki examined the asymptotic behavior of global solutions to a forest kinetic model, which is structured into populations of young trees, old trees, and airborne seeds. The analysis establishes the convergence of these solutions to a stationary state under a specified set of parameter conditions. The proof leverages two principal components: the establishment of a non-smooth variant of the Lojasiewicz–Simon gradient inequality within a suitably chosen functional space, and the derivation of specific norm estimates for the time derivative of the global solutions. The combination of these tools provides a framework for concluding the long-term stabilization of the system’s dynamics [4].
Lu and Cantinthe studied asymptotic dynamics of a degenerate forest kinematic model under climate change-induced perturbations. It establishes that, when the main nonlinear term is monotone, global solutions converge to a stationary state by proving that the system’s Lyapunov function satisfies a Łojasiewicz–Simon gradient inequality. The authors further propose a statistical model checking algorithm to estimate convergence probabilities toward non-constant equilibria. Analytical results demonstrate the continuity of the flow and stationary solutions with respect to the perturbation parameter, alongside the robustness of weak attractors through positively invariant regions in a weak topology phase space. Numerical simulations supplement the theoretical analysis, revealing that the model can also exhibit chaotic patterns under certain perturbations [5].
The original model adopted Dirichlet boundary conditions; however, since the dispersal of seeds and trees in nature seldom approaches a fixed value at the domain edge, we instead impose Neumann boundary conditions to reflect the flux across the boundary. Our present work seeks to extend this framework by introducing diffusion processes for distinct adult age classes (e.g., young and old trees). The rationale for this inclusion is twofold. First, from a mechanistic perspective, while individual adult trees are stationary, population-level spatial redistribution occurs through processes such as localized recruitment (e.g., seeds germinating near parent trees, effectively creating a short-range “diffusive” shift in the center of a cohort), small-scale gap-phase replacement, or very slow clonal spread. These processes can be meaningfully aggregated into a phenomenological diffusion term at the population scale, especially when modeling larger spatial or temporal domains. Second, from a dynamical systems standpoint, including diffusion for all state variables, allows for a complete analysis of spatial instability mechanisms, such as Turing patterning, which requires differential diffusion rates among interacting components. By endowing adult classes with their own (typically smaller) diffusion coefficients, we can investigate whether age-structured spatial fluxes, interacting with seed diffusion, can generate novel spatial patterns or stability properties not observed in models where only seeds diffuse.
A significant body of research has been dedicated to analyzing the asymptotic behavior of solutions to the forest kinematic model under various boundary conditions [6,7,8]. Studies have established the existence of global solutions, constructed dynamical systems, and investigated the stability of equilibrium points [6,7].
Furthermore, the model’s capacity for pattern formation, a classic topic in theoretical ecology since Turing’s seminal work [9], has been explored. Turing instability, whereby diffusion drives a stable homogeneous equilibrium to become unstable and yield spatially heterogeneous patterns, has been extensively studied in ecological contexts, including predator–prey systems [10] and competing species models [11]. However, the dynamics become significantly richer when the system exhibits temporal oscillations before spatial patterning occurs. This leads to the phenomenon of Turing instability of Hopf bifurcation-induced periodic solutions. In this scenario, a spatially uniform steady state loses stability via Hopf bifurcation, giving rise to stable, spatially homogeneous periodic oscillations. Subsequently, diffusion can destabilize these temporal oscillations, leading to complex spatiotemporal patterns such as traveling waves or phase patterns [12,13]. The interplay between time delay, diffusion, and nonlinearity has been shown to induce Hopf bifurcations in various ecological models, underscoring the richness of dynamics in spatiotemporal systems [14]. Hou and Sun investigated vegetation pattern transitions in arid and semi-arid ecosystems, shifting the focus from natural drivers to active human intervention. By integrating optimal control theory into the Rietkerk model, the study introduces controllable human activities as control variables to analyze and direct pattern formation. The primary findings indicate that even under unfavorable environmental conditions, strategically designed spatiotemporal distributions of human intervention can successfully induce the desired pattern transitions. Furthermore, the research demonstrates that incorporating sparsity constraints within an acceptable error margin can significantly reduce control costs without compromising transition effectiveness. Overall, this study proposes a control-theoretic framework for analyzing and facilitating vegetation pattern transitions, contributing a methodological perspective for developing strategies in desertification control and ecosystem restoration [15].
Concurrently, empirical and theoretical ecology has increasingly emphasized the pivotal role of tree mortality mechanisms in shaping forest structure and dynamics, including the critical role of animal-mediated seed dispersal for global plant migration under climate change. The authors develop trait-based models to predict pairwise plant–animal interactions and estimate dispersal function for fleshy-fruited plants worldwide. By using interactions with introduced species as a proxy for future novel networks, the research demonstrates the feasibility of forecasting the assembly and function of these changing ecological partnerships [16]. For instance, research in Canadian boreal forests and mixed European stands has demonstrated that temperature increases and drought stress significantly elevate mortality risk for many species [17,18]. Moreover, niche marginality studies reveal that trees are more vulnerable to mortality from hotter-drought events when they are at the edge of their climatic niche, particularly for gymnosperms [19]. These findings highlight that tree mortality is not a simple constant but a complex, often density- and climate-dependent process, justifying the incorporation of a sophisticated function like in the forest kinematic model. Parameter b in this function, representing the optimal density for sapling survival, can be interpreted as an aggregate reflection of competitive balance and resource availability, factors known to be sensitive to climate conditions [17,18].
Despite these advances, a critical gap remains in synthesizing these two fronts: the sophisticated mathematical analysis of pattern formation and the empirically grounded understanding of nonlinear mortality processes. While some studies have touched upon the dynamics of reaction–diffusion systems with nonlinear interactions [10,11,20], the specific investigation of how a density-dependent mortality rate, particularly one with a parabolic structure like , can act as a Hopf bifurcation parameter and subsequently facilitate the Turing instability of the resulting periodic solutions in a forest model, is largely unexplored. This gap is significant because such a mechanism could provide a novel theoretical pathway for spatial pattern formation in forests, distinct from the classic Turing mechanism applied to equilibria. It aligns with the growing recognition that environmental changes can alter key demographic rates, such as mortality, which in turn can trigger large-scale ecological transitions [21]. Ge examined the long-range spatial properties of vegetation Turing patterns in arid and semi-arid ecosystems. By drawing an analogy to hyperuniform structures from material science, they found that these patterns exhibit a characteristic long-range dispersion akin to hyperuniformity. The analysis establishes a positive correlation between the degree of pattern hyperuniformity and vegetation water-use efficiency, supporting the view of Turing patterns as spatially optimized configurations for resource acquisition. Furthermore, the work identifies that the degree of hyperuniformity demonstrates critical slowing down near ecological tipping points and serves as an indicator of spatial resilience. It shows that disturbances which reduce pattern hyperuniformity lead to significantly longer recovery times compared to those that preserve it [22].
Therefore, this paper aims to bridge this gap by conducting a thorough nonlinear analysis of the diffusive forest kinematic model, with a special focus on the role of the mortality function . Our primary objectives are as follows:
To analyze the stability of the positive equilibrium and identify the conditions under which parameter b in acts as a Hopf bifurcation parameter, leading to spatially homogeneous periodic solutions.
To derive the criteria for Turing instability of the periodic solutions arising from the Hopf bifurcation, induced by the diffusion of seeds.
To numerically simulate the resulting spatiotemporal patterns and discuss their potential ecological implications for forest patch dynamics.
This investigation is not only mathematically intriguing but also ecologically relevant. It provides a theoretical foundation for understanding how subtle changes in density-dependent feedback mechanisms, potentially driven by climate change [17,19], can precipitate large-scale spatial reorganization in forest ecosystems. By integrating advanced dynamical systems theory with empirically motivated biology, this study contributes to a more predictive understanding of forest dynamics in a changing world.
We will apply our result on the parameter space . Parameter b relates to the mortality of young trees that are minimized at a specific old tree density, whereas is the seed deposition rate.
Here, we establish explicit thresholds for Turing instability that emerge directly from a Hopf bifurcating periodic orbit in system (2). The highlights are as follows:
- 1.
- Closed-form Hopf criterion: The first algebraic conditions on the kinetic parameters that guarantee a super-critical oscillatory bifurcation.
- 2.
- Turing–Hopf overlap: A simultaneous stability diagram showing where the same periodic solution loses spatial stability—no extra constraints or auxiliary systems required.
- 3.
- Predictive formulae: Explicit wavenumber intervals and diffusion ratios that trigger patterning on the limit cycle, verified by spectral computations and time-stepping simulations.
These results supply designers of reaction–diffusion models with ready-to-use formulae to switch from global oscillations to stable spatial patterns without retuning parameters.
2. Hopf Bifurcations in the Forest Kinematic Model
In this section, we consider the stability and Hopf bifurcations in the forest kinematic model, which had been proposed as following ODE form:
here we also assumed that is a square function which has a minimum at some value of v, namely, .
2.1. Existence of the Hopf Bifurcation in the Forest Kinematic ODE Model
Firstly, for determining that Hopf bifurcation exists in the forest kinematic ODE model, the following deduction was based on the conditions of Hopf bifurcation.
Clearly, system (3) has and positive equilibrium solution , where . And is given by
so we have
where .
There are some cases of as follows. We shall select b as the bifurcation parameter. Then, the linearized operator evaluated at is given by
where we use the fact that . The characteristic equation of is given by
where
First, we set and by examining the sign of , we further clarify the cases of the equilibrium stability and the possible emergence of Hopf bifurcation under different parameter cases.
Case 1: When , no Hopf bifurcation occurs because the equilibrium remains locally asymptotically stable under this condition, and we have .
We also observe that ; thus, . Then we obtain , .
Hence , concurrently we have
While , we can obtain ; however, are fixed. For any , is satisfied. Therefore, when , we have , and then this solution is always locally asymptotically stable.
Case 2: When , namely, , to ensure positive roots exist. Set ; we discuss the following subcases:
(1) If , then both and are positive roots.
(2) If , then is a positive root, and the negative root is discarded.
When , the calculation shows that
and we have
where
From , it follows that there are two roots, given by
Since , we have for . Therefore, as , is always locally asymptotically stable.
Finally, considering as the positive root of the Equation (5), it is necessary to satisfy ; meanwhile, it should satisfy . Combine it with , i.e., .
Thus, we can deduce that , but the signs of , and require further discussion.
where
From , we have
From , we have
From , we can obtain
Based on the above discussion, we obtain the following conclusions:
Proposition 1.
Let , , and be defined in (12), (13), and (14). And , and . Then, the following conclusions hold true:
- Suppose that holds. Then, for , when , is unstable; when , is always locally asymptotically stable.
- Suppose that holds. Then, for , when , is unstable; when , is always locally asymptotically stable. Only when does the ODEs system (3) undergo Hopf bifurcation around .
Proof.
The proof is trivial and we shall omit the proof. □
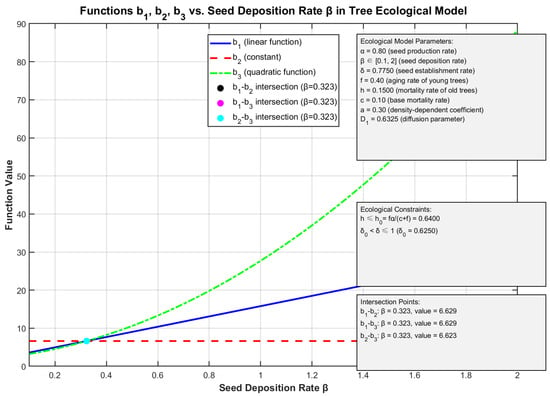
To isolate the effect of parameter , for example, we fixed , , , . The results of this configuration are presented in Figure 1, which reveals that Hopf bifurcation occurred on the green curve of over the red and blue line of in the first quadrant with .
Figure 1.
Hopf bifurcation occurred on the green curve of over the blue and red line of in the first quadrant.
2.2. Direction of Hopf Bifurcation and Stability of the Periodic Solutions
Now, we are in a position to state the following results on the stability/instability of with respect to the ODEs system (3).
Theorem 1.
Let , and be defined in Proposition 1. Then, the following conclusions hold true:
Proof.
According to Proposition 1, the stability of the equilibrium is determined by the parameters and b as follows:
When or , the equilibrium is unstable.
When or , the equilibrium is locally asymptotically stable.
Now, consider the case and . According to Proposition 1, the ODE system (3) undergoes Hopf bifurcation around at . To verify the conditions for Hopf bifurcation, we examine the behavior of the eigenvalues at . Let the characteristic equation be
At , there exists a pair of purely imaginary roots (with ) and one negative real root. The transversality condition requires
Based on the analysis in Proposition 1, when , the transversality condition holds at (since for ). Specifically, in case 2 (i.e., ), at , we have , which ensures the transversality condition is satisfied.
Therefore, based on the Hopf bifurcation theorem (Theorem A.1 in [23]), there exists such that for , there exists a bifurcation parameter (with ) and a periodic solution with minimal period , satisfying as .
This completes the proof of the theorem. □
Remark 1.
For brevity and clarity, for any fixed , we denote and by and P, respectively.
Theorem 2.
Let , and be defined in Proposition 1. Suppose that . Then, the Hopf bifurcation at is supercritical and forward (resp., subcritical and backward) if (resp., ), where is precisely defined in (19).
Proof.
By Theorem A.1 of [23], to study the Hopf bifurcation direction and the stability of the bifurcating periodic solutions, we need to consider the sign of .
We shall calculate by using the general framework of Theorem A.1 of [23]. To that end, we define the matrix P in the following way:
where , , . Now according to the paper [23], we also define
where is the determinant of P and
where
Then, by (A.17) in Appendix of [23], we have
where , and are defined in (18).
By Theorem 1, and Theorem A.1 of paper [23], Hopf bifurcation at is supercritical and forward (resp., subcritical and backward) if (resp., ). Furthermore, by Theorem 1, we have . □
3. The Dynamics of the Forest Kinematic PDE System
According to the results in [23], the following lemma can be obtained:
Lemma 1.
Suppose that there exists some , so that , and that
Then, we have
- 1.
- For any sufficiently small , when , is stable; while , is unstable if
- 2.
- For any sufficiently small , when , is unstable; while , is stable if
- 3.
- At , system (3) undergoes Hopf bifurcation around . Here , is a periodic solution bifurcating from Hopf bifurcation. In addition, bifurcation is supercritical if , and is backward ifwhen the bifurcation is subcritical if , and is forward ifwhere denotes the first Lyapunov coefficient and stands for the real parts of .
Furthermore, Wang and Yi [23] also provide conditions on so that Turing instability of the periodic solutions occurs.
Lemma 2.
Suppose that λ is fixed to be sufficiently close to so that is a stable periodic solution of the ODE system (3) bifurcating from at , as stated in Theorem 1. Then, is unstable with respect to the reaction–diffusion system (2) if Ω is large enough, and
where
Turing Instability of the Hopf Bifurcating Spatially Homogeneous Periodic Solutions
In this subsection, we are in the position to use Theorem A.5 in Appendix of paper [23] or other recent literature [24,25,26,27,28,29,30] to study Turing instability of in the reaction–diffusion system (2):
Theorem 3.
Let λ be fixed to be sufficiently close to so that is a stable (in the sense that ) Hopf bifurcating periodic solution of system (3). Then, will undergo Turing instability if ℓ is sufficiently large and
where , , and are defined in (10), is denoted in cases 2, such as when , let , and is given by
where is defined in (19) and
4. Numerical Simulations
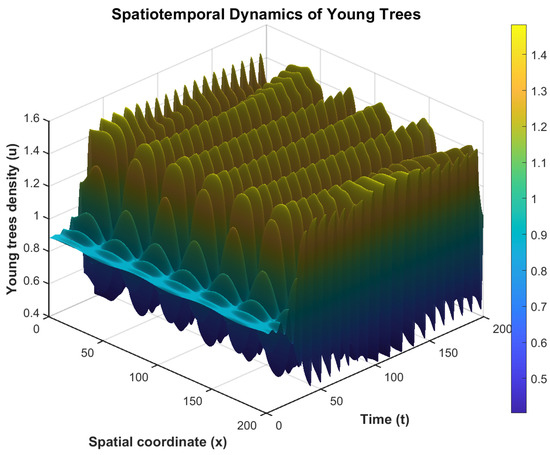
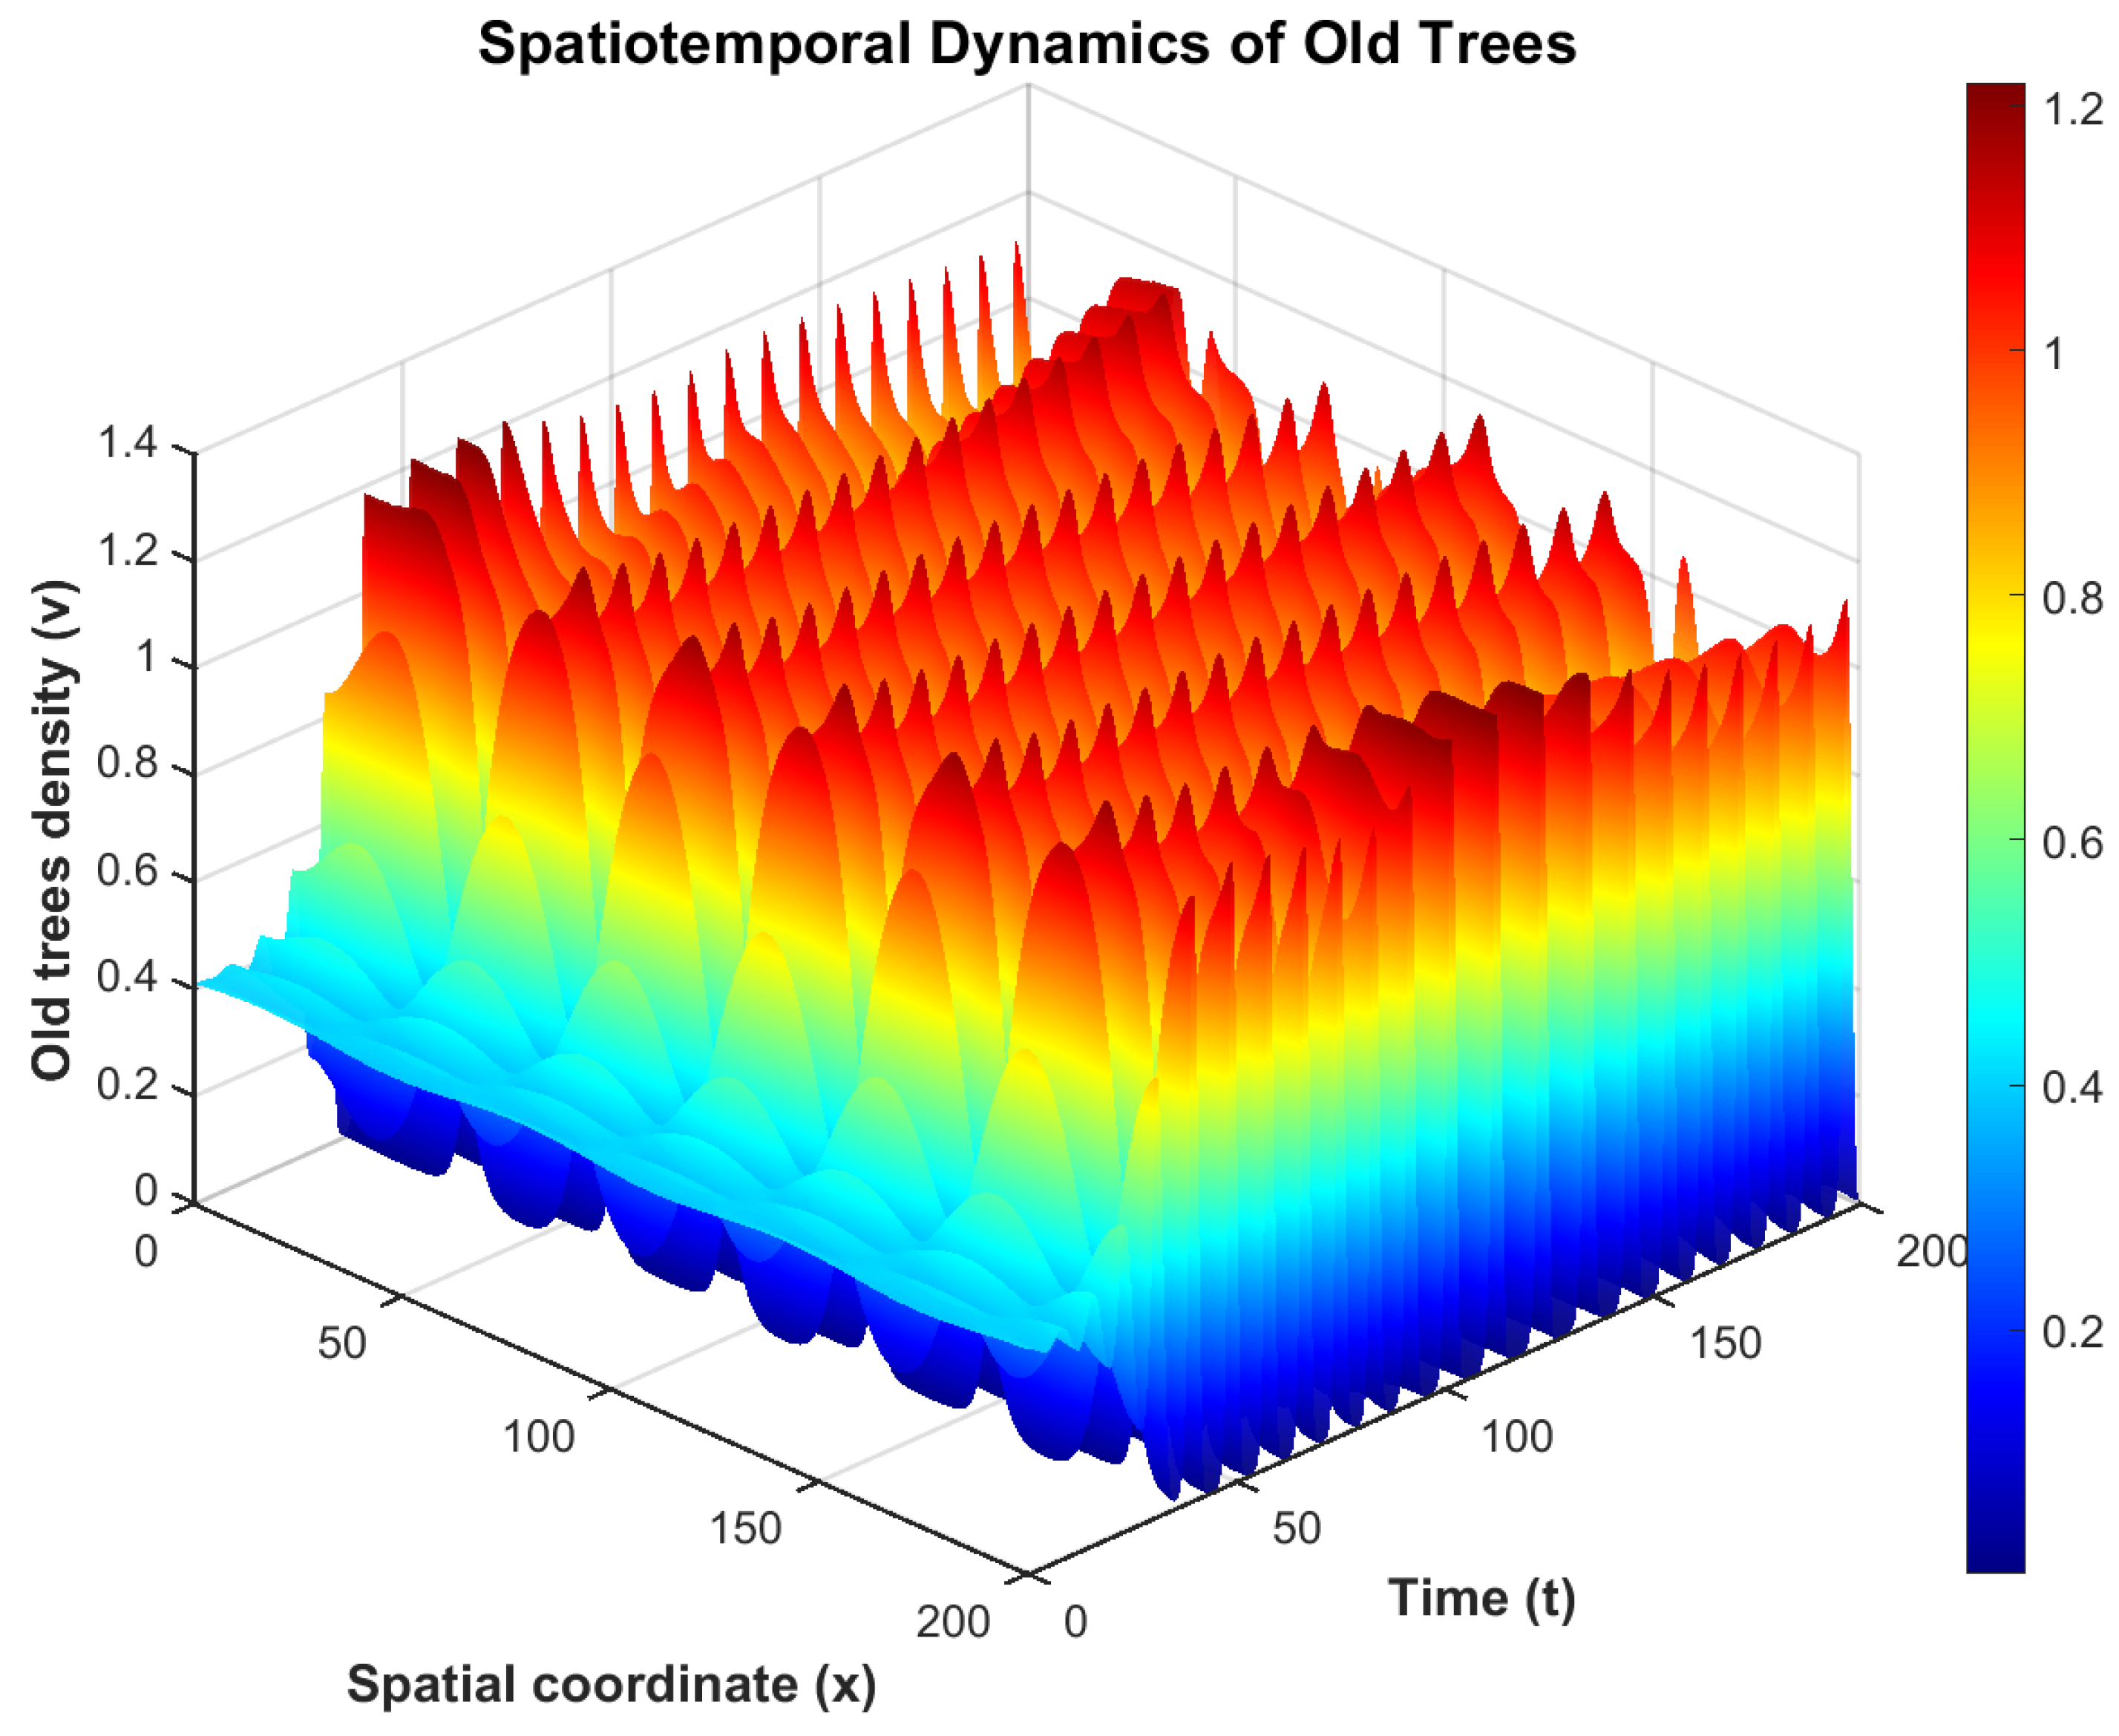
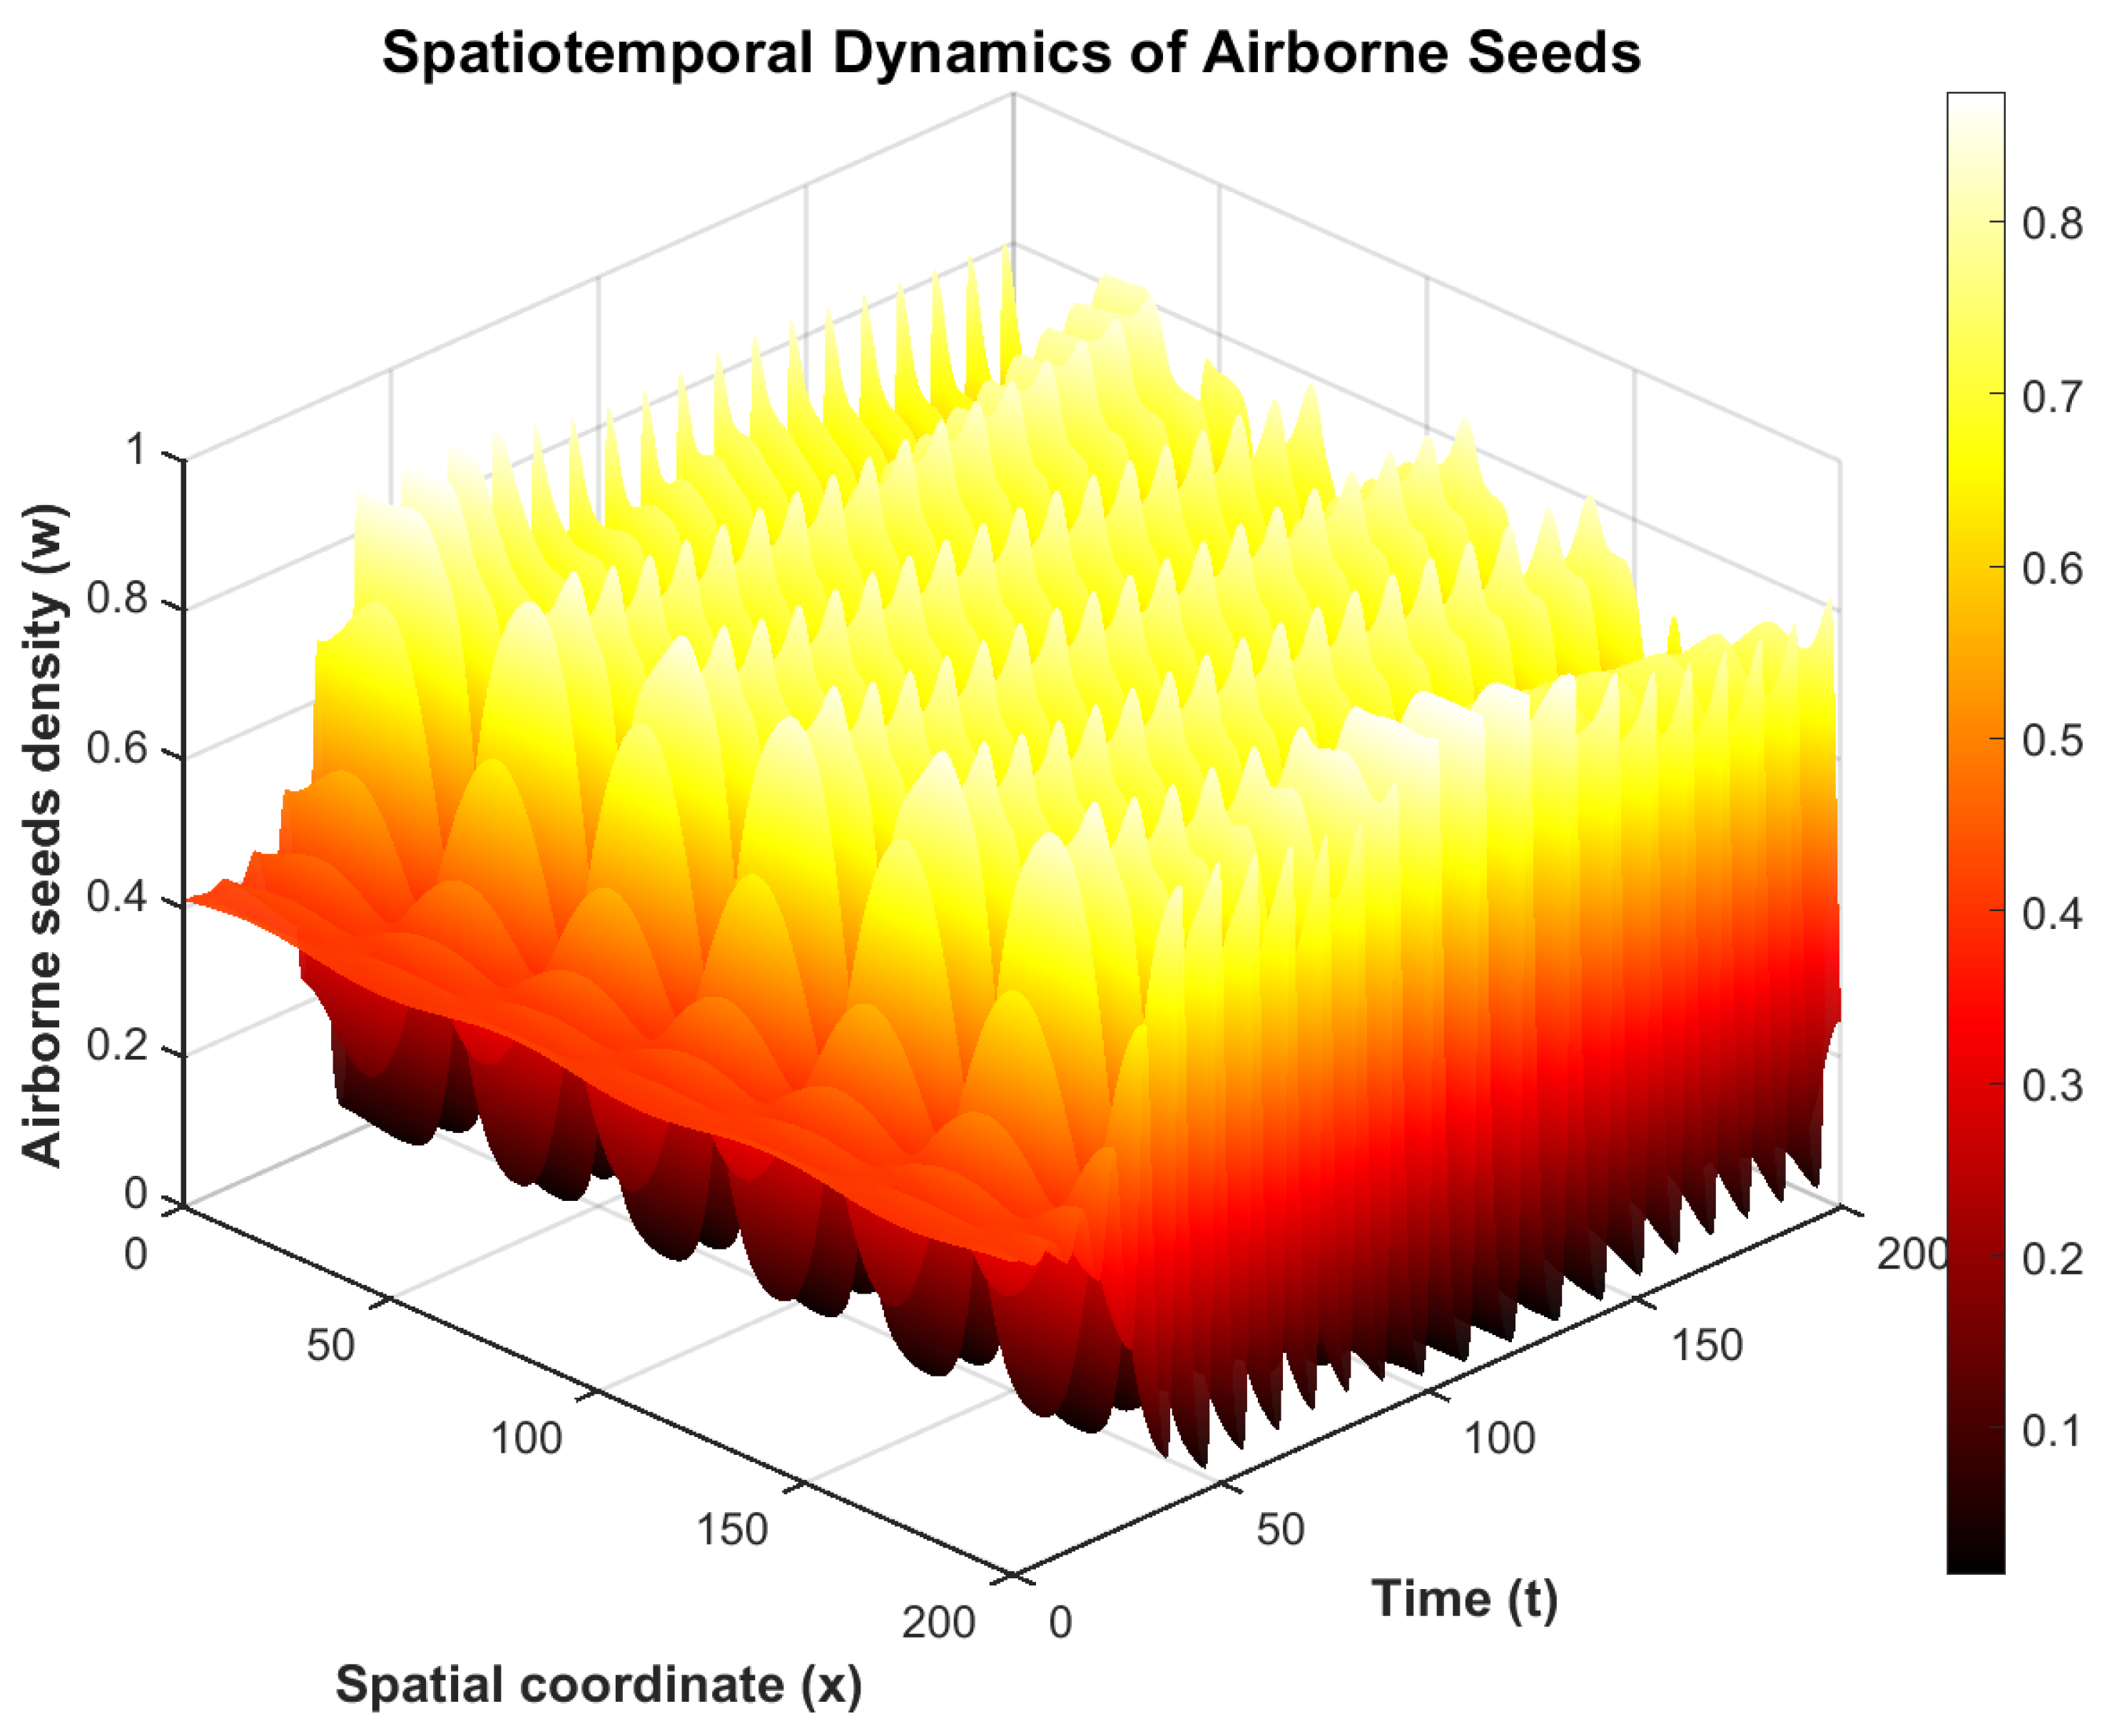
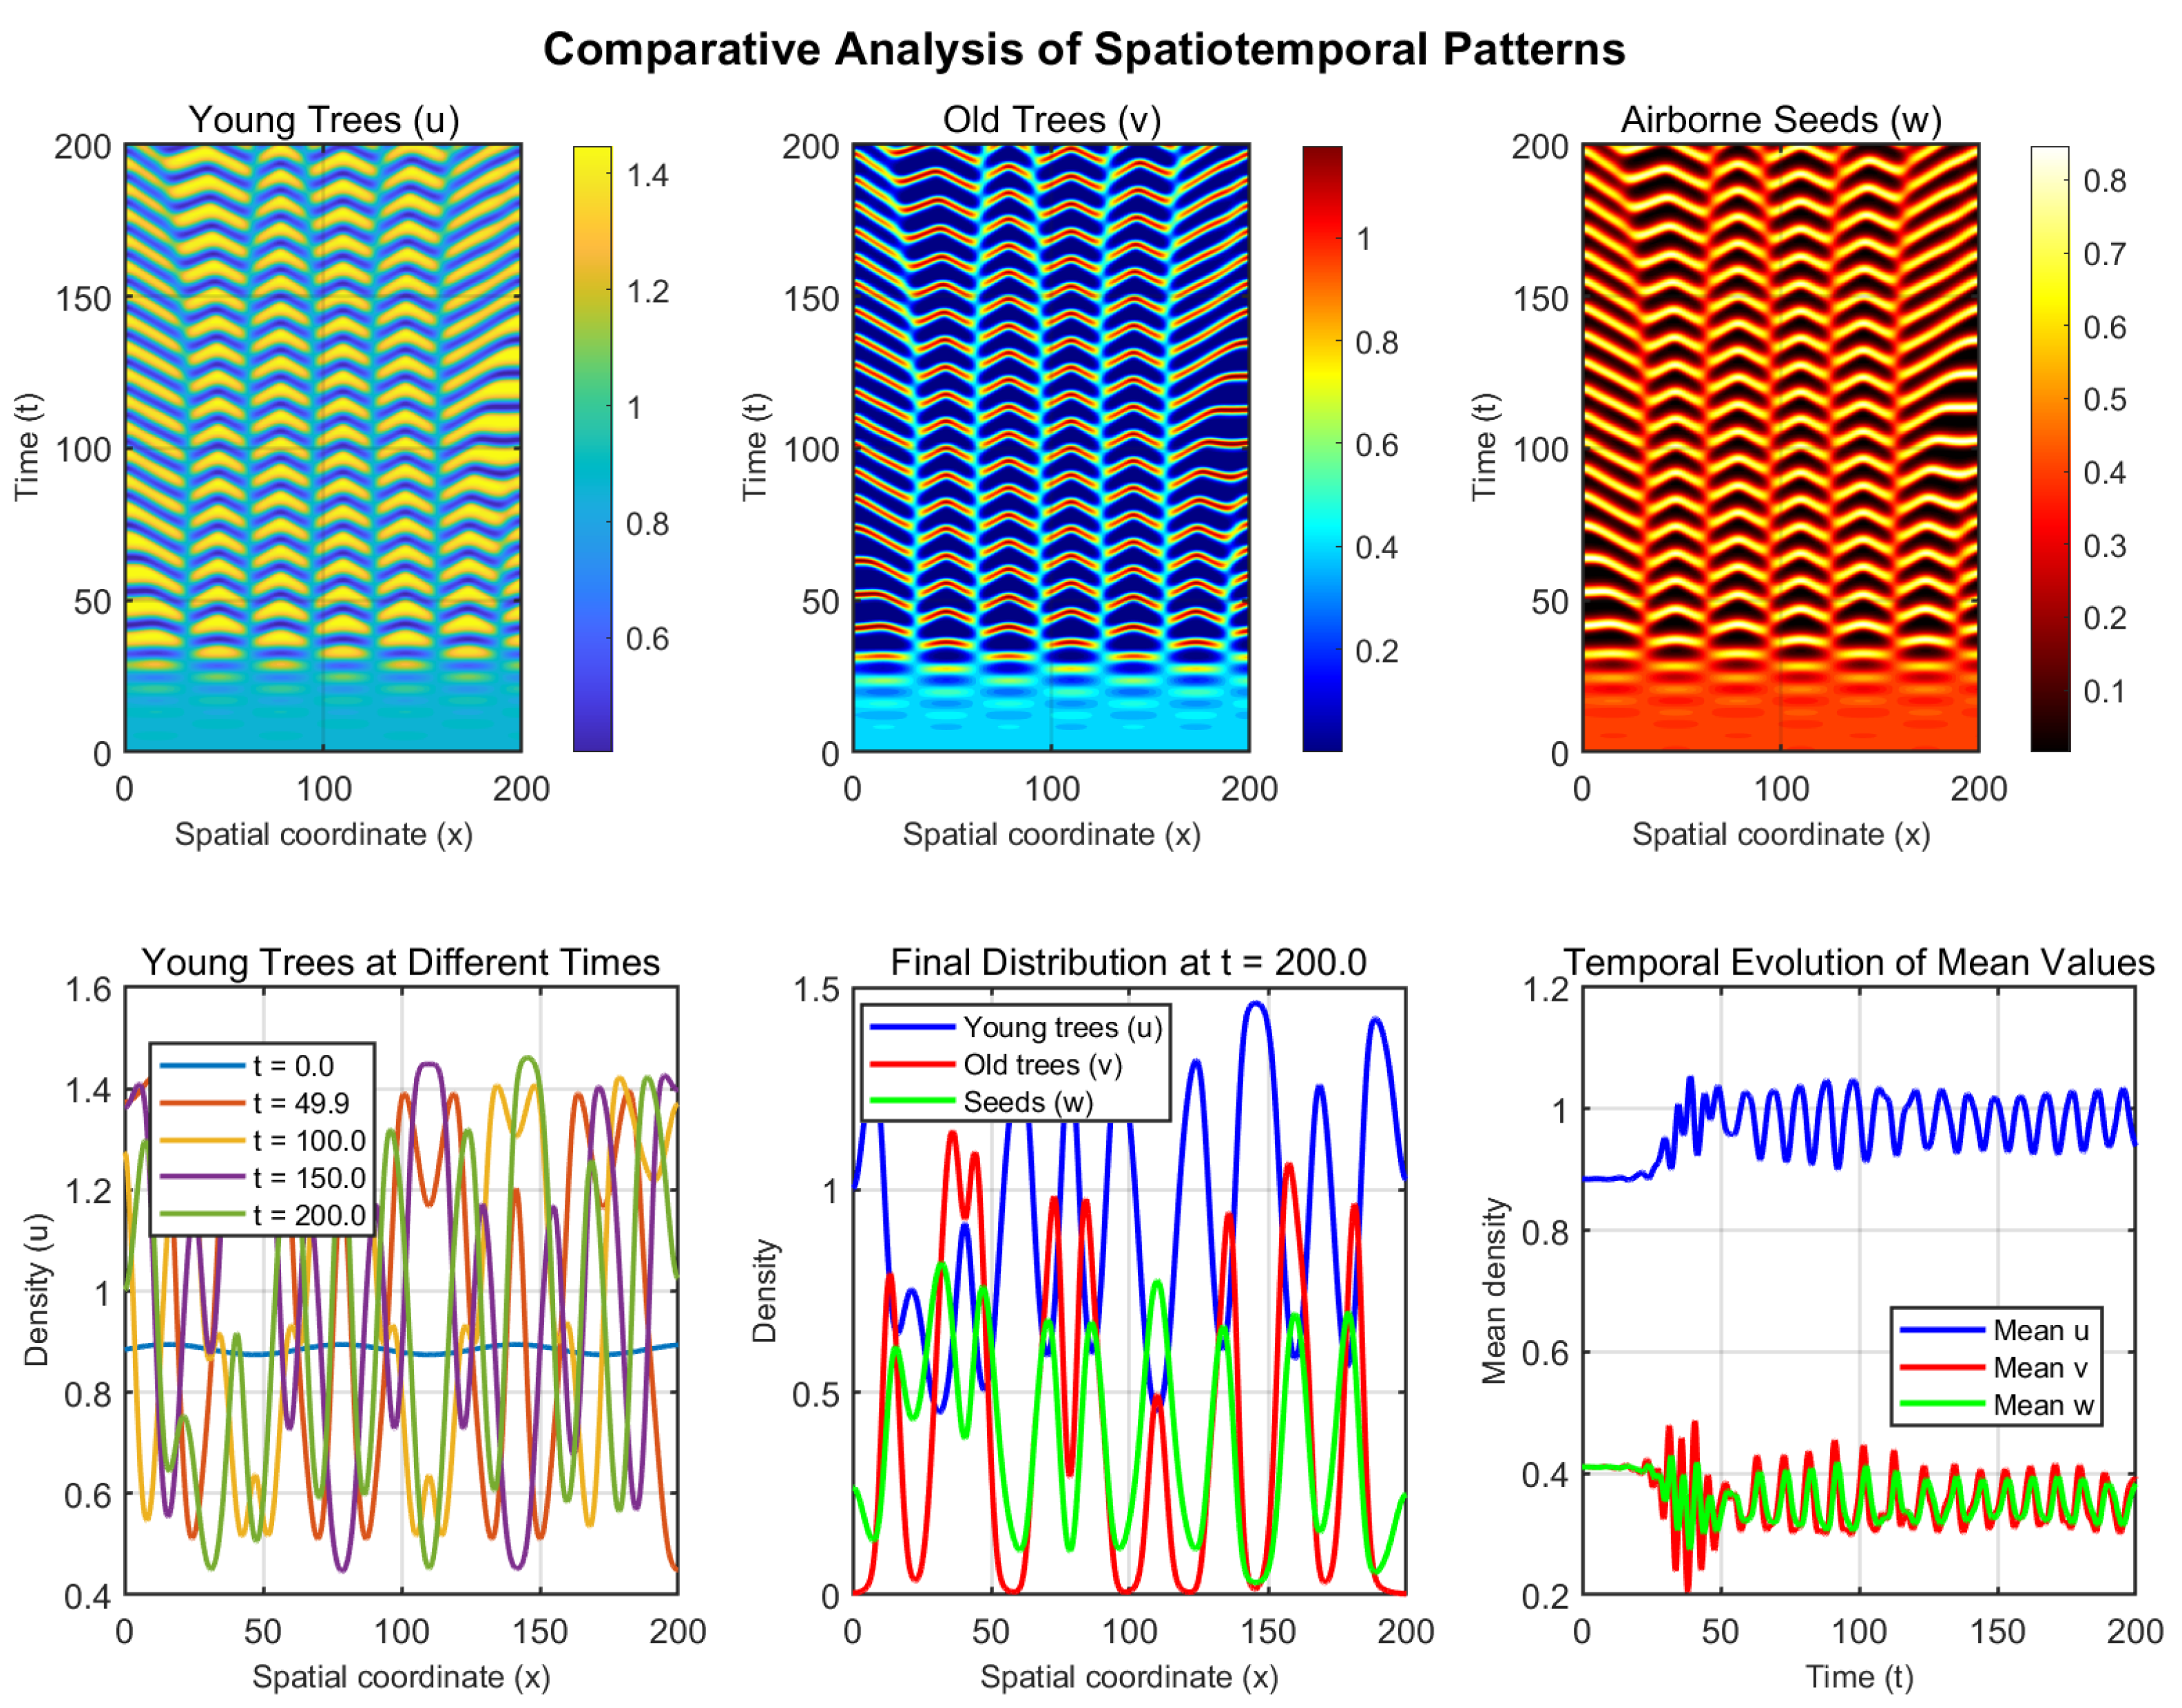
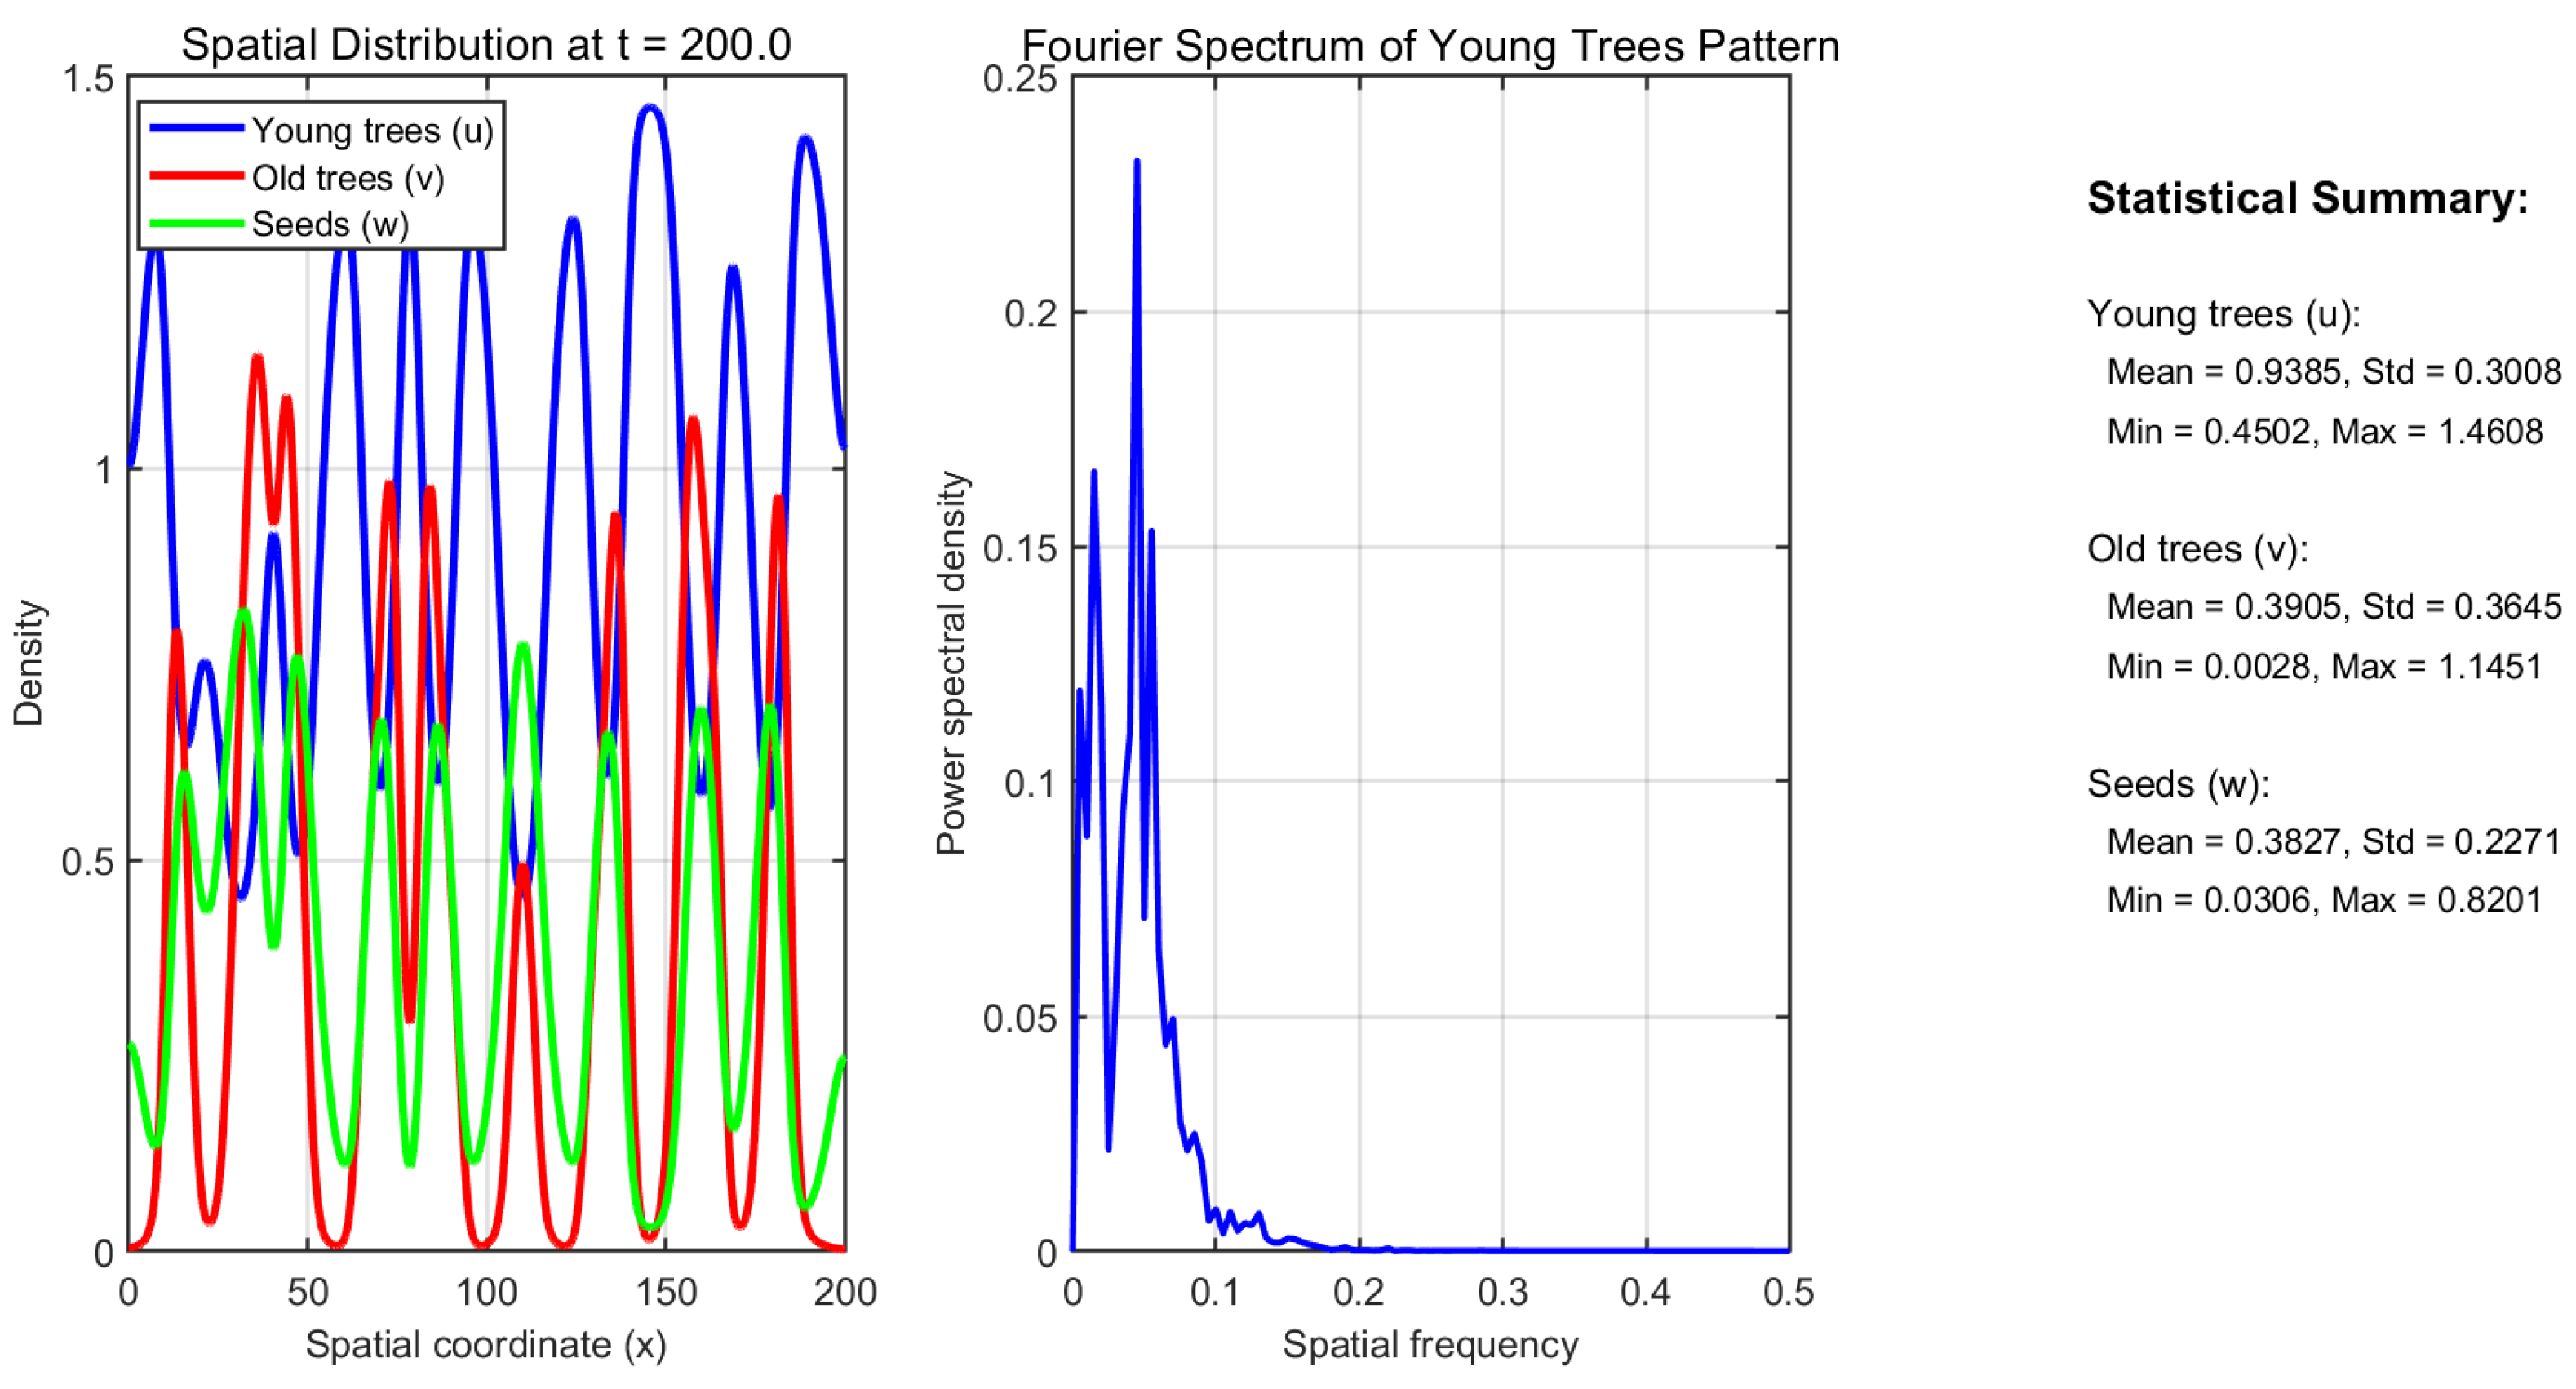
In this section, we present numerical simulations to validate the theoretical findings regarding Hopf bifurcation and Turing instability derived in Section 2 and Section 3. The PDE system (2) is solved using the method of lines with finite difference spatial discretization and adaptive time stepping. Neumann boundary conditions are imposed to simulate an isolated spatial domain. Initial conditions are set as the homogeneous equilibrium perturbed by a small-amplitude sinusoidal function. The resulting spatiotemporal dynamics are visualized in Figure 2, Figure 3, Figure 4, Figure 5 and Figure 6.
Figure 2.
Spatiotemporal evolution of the tree densities showing homogeneous temporal oscillations after Hopf bifurcation. The solution remains spatially uniform, consistent with the theoretical prediction of a spatially homogeneous limit cycle.
Figure 3.
The emergence of spatially modulated patterns due to Turing instability of the Hopf-induced periodic solution. The system transitions from uniform oscillations to a spatially patterned state, illustrating the interaction between temporal and spatial instabilities.
Figure 4.
Contour plots, time slices, and mean trajectories under different diffusion coefficients. From left to right: homogeneous oscillations; stable Turing patterns; complex spatiotemporal chaos.
Figure 5.
The figures depict the stability diagram in the plane, the spatial Fourier spectrum and the statistical measures of pattern formation.
Figure 6.
Two-dimensional Turing patterns emerging from the Hopf-induced periodic state. Patterns exhibit either spotted or striped morphology depending on diffusion coefficients and domain size.
Figure 2 illustrates the temporal evolution of the system in a one-dimensional spatial domain when the parameters lie near the Hopf bifurcation curve derived in Proposition 1. After a small perturbation to the homogeneous steady state, the system exhibits spatially uniform temporal oscillations, confirming the occurrence of a supercritical Hopf bifurcation, as predicted by Theorem 1. This spatially homogeneous periodic solution serves as the base state for the subsequent Turing instability analysis.
When diffusion coefficients satisfy condition (23) in Theorem 3, the spatially homogeneous periodic solution loses stability and gives rise to spatially modulated patterns. Figure 3 demonstrates this transition, where diffusion-induced inhomogeneities lead to the formation of standing wave patterns. This numerical observation confirms that diffusion can destabilize temporal oscillations, leading to Turing instability on the limit cycle—a key finding of this study.
Figure 4 provides a comparative analysis of spatiotemporal dynamics under three distinct sets of diffusion coefficients . Contour plots, time slices, and mean trajectories reveal how the relative magnitudes of diffusion rates influence pattern formation. The left panel corresponds to nearly equal diffusion coefficients, resulting in sustained homogeneous oscillations. The middle panel shows the emergence of stable Turing patterns when (seed diffusion) dominates. The right panel exhibits complex spatiotemporal chaos when diffusion rates are tuned beyond the instability threshold. These results underscore the critical role of differential diffusion in driving spatial self-organization.
Figure 5 depicts the stability regions in the parameter space, with the green area indicating stable periodic solutions and the red area marking the Turing unstable regime. Figure 5 shows the spatial Fourier spectrum of the emergent pattern, with a distinct peak at the dominant wavenumber , corresponding to a characteristic wavelength of approximately 14 spatial units. Figure 5 lists basic statistics, including spatial standard deviations exceeding 10, confirming significant spatial heterogeneity induced by diffusion.
Figure 6 extends the simulation to a two-dimensional domain, revealing the formation of spotted and striped patterns reminiscent of vegetation self-organization observed in dryland ecosystems. These patterns not only validate the theoretical predictions of Turing–Hopf bifurcation in higher spatial dimensions but also suggest potential ecological implications for forest patchiness under environmental stress.
The numerical simulations collectively confirm the theoretical framework developed in this paper: parameter b in the mortality function acts as a Hopf bifurcation parameter, leading to homogeneous oscillations; diffusion then destabilizes these oscillations via the Turing mechanism, giving rise to spatially organized patterns. These findings provide a mechanistic explanation for how density-dependent mortality and seed dispersal can jointly drive spatiotemporal patterning in forest ecosystems.
5. Conclusions
This paper investigates the Turing instability of spatially homogeneous Hopf bifurcating periodic solutions in a diffusive forest kinematic model. Thus, the research results of this paper enrich the dynamic theoretical framework of the forest system model, and hold particular significance for analyzing the stability of periodic solutions under the combined effects of spatial diffusion and environmental perturbations. In the future, the study can be further extended to higher-dimensional spatial structures or multi-parameter disturbance scenarios to more comprehensively understand the complex spatiotemporal evolution mechanisms of vegetation dynamics in forest ecosystems.
Beyond the theoretical insights, our study offers an ecological perspective on how density-dependent feedbacks mediated by tree mortality can drive spatial self-organization in forests. The discussion on the allometric relationship between leaf area and stem cross-sectional area underscores the potential of our model to bridge mathematical abstraction with real forest structure dynamics. Such relationships may help explain observed spatial patterns in forest stands, where resource allocation and competition interact with dispersal to shape patchiness. Future work could integrate empirical data on tree allometry and mortality to calibrate the functional form of the mortality rate, enabling more predictive scenarios under climate change. Moreover, extending the model to include spatial heterogeneity in resource availability or multi-species interactions would further enhance its applicability to real-world forest ecosystems.
Author Contributions
Software, W.Z.; formal analysis, Y.H.; writing—original draft, J.Y.; writing—review and editing, M.W.; supervision, M.W. All authors have read and agreed to the published version of the manuscript.
Funding
This research was funded by the Northeast Forestry University College Student Innovation and Entrepreneurship Training Program Project: 202510225636; the Fundamental Research Funds for the Central Universities: 60201523050.
Data Availability Statement
The original contributions presented in this study are included in the article. Further inquiries can be directed to the corresponding author.
Conflicts of Interest
The authors declare no conflicts of interest.
References
- Kuznetsov, Y.; Antonovsky, M.; Biktashev, V.; Aponina, A. A cross-diffusion model of forest boundary dynamics. J. Math. Biol. 1994, 32, 219–232. [Google Scholar] [CrossRef] [Scilit]
- Shirai, T.; Chuan, L.; Yagi, A. Asymptotic behavior of solutions for forest kinematic model under Dirichlet conditions. Sci. Math. Japon. 2007, 66, 289–301. [Google Scholar] [CrossRef] [Scilit]
- Chuan, L. Asymptotic Behavior of Solutions for Forest Kinematic Model. Funkcial. Ekvac. 2006, 49, 427–449. [Google Scholar] [CrossRef] [Scilit]
- Satoru, I. Asymptotic convergence of solutions to the forest kinematic model. Nonlinear Anal. Real World Appl. 2021, 62, 103382. [Google Scholar] [CrossRef] [Scilit]
- Lu, L.; Cantin, G. Asymptotic Behavior of a Degenerate Forest Kinematic Model with a Perturbation. Stud. Appl. Math. 2025, 154, 1–21. [Google Scholar] [CrossRef] [Scilit]
- Chuan, L.; Yagi, A. Dynamical system for forest kinematic model. Adv. Math. Sci. Appl. 2006, 2, 16. [Google Scholar]
- Chuan, L.; Tsujikawa, T.; Yagi, A. Stationary solutions to forest kinematic model. Glasg. Math. J. 2009, 51, 1–17. [Google Scholar] [CrossRef] [Scilit]
- T’Emam, R. Infinite-Dimensional Dynamical Systems in Mechanics and Physics; Springer Science & Business Media: New York, NY, USA, 2012. [Google Scholar]
- Turing, A. The chemical basis of morphogenesis. Philos. Trans. R. Soc. Lond. B Biol. Sci. 1952, 237, 37–72. [Google Scholar] [CrossRef] [Scilit]
- Murray, J. Mathematical Biology II: Spatial Models and Biomedical Applications, 3rd ed.; Springer: Berlin/Heidelberg, Germany, 2003. [Google Scholar]
- Volpert, A.; Petrovskii, S. Reaction-diffusion waves in biology. Phys. Life Rev. 2009, 6, 267–310. [Google Scholar] [CrossRef] [Scilit]
- Ouyang, Q.; Swinney, H. Transition from a uniform state to hexagonal and striped Turing patterns. Nature 1991, 352, 610–612. [Google Scholar] [CrossRef] [Scilit]
- Cross, M.; Hohenberg, P. Pattern formation outside of equilibrium. Rev. Mod. Phys. 1993, 65, 851. [Google Scholar] [CrossRef] [Scilit]
- Chen, S.; Lou, Y.; Wei, J. Hopf bifurcation in a delayed reaction-diffusion-advection population model. J. Differ. Equ. 2018, 264, 5333–5359. [Google Scholar] [CrossRef] [Scilit]
- Hou, L.; Wang, S.; Li, L.; Li, B.; Sun, G. Spatiotemporal complexity of vegetation dynamics in view of optimal control. Physica A 2025, 680, 131028. [Google Scholar] [CrossRef] [Scilit]
- Fricke, E.; Ordonez, A.; Rogers, H.; Svenning, J. The effects of defaunation on plants’ capacity to track climate change. Science 2022, 375, 6. [Google Scholar] [CrossRef] [Scilit]
- Zhou, G.; Peng, C.; Li, Y.; Liu, S.; Zhang, Q.; Tang, X.; Liu, J.; Yan, J.; Zhang, D.; Chu, G. A climate change-induced threat to the ecological resilience of a subtropical monsoon evergreen broad-leaved forest in Southern China. Glob. Change Biol. 2013, 19, 1197–1210. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pretzsch, H.; Schütze, G.; Uhl, E. Resistance of European tree species to drought stress in mixed versus pure forests: Evidence of stress release by inter-specific facilitation. Plant Biol. 2013, 15, 483–495. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tabarelli, M.; Aguiar, A.V.; Ribeiro, M.C.; Metzger, J.P.; Peres, C.A. Prospects for biodiversity conservation in the Atlantic Forest: Lessons from aging human-modified landscapes. Biol. Conserv. 2010, 143, 2328–2340. [Google Scholar] [CrossRef] [Scilit]
- Ghergu, M.; Vicenţiu, D. Rădulescu, Nonlinear PDEs: Mathematical Models in Biology, Chemistry and Population Genetics; Springer Science & Business Media: New York, NY, USA, 2011. [Google Scholar]
- Scheffer, M.; Carpenter, S.; Foley, J.A.; Folke, C.; Walker, B. Catastrophic shifts in ecosystems. Nature 2001, 413, 591–596. [Google Scholar] [CrossRef] [Scilit]
- Ge, Z. The hidden order of Turing patterns in arid and semi-arid vegetation ecosystems. Proc. Natl. Acad. Sci. USA 2023, 120, 11. [Google Scholar] [CrossRef] [Scilit]
- Wang, M.; Yi, F. On the dynamics of the diffusive Field-Noyes model for the Belousov-Zhabotinskii reaction. J. Differ. Equ. 2022, 318, 443–479. [Google Scholar] [CrossRef] [Scilit]
- Li, S.; Wu, J.; Dong, Y. Turing patterns in a reaction-diffusion model with the Degn-Harrison reaction scheme. J. Differ. Equ. 2015, 259, 1990–2029. [Google Scholar] [CrossRef] [Scilit]
- Satnoianu, R.; Menzinger, M.; Maini, P. Turing instabilities in general systems. J. Math. Biol. 2000, 41, 493–512. [Google Scholar] [CrossRef] [Scilit]
- Yi, F.; Wei, J.; Shi, J. Bifurcation and spatiotemporal patterns in a homogenous diffusive predator-prey system. J. Differ. Equ. 2009, 246, 1944–1977. [Google Scholar] [CrossRef] [Scilit]
- Yi, F. Turing instability of the periodic solutions for reaction-diffusion systems with cross-diffusion and the patch model with cross-diffusion-like coupling. J. Differ. Equ. 2021, 281, 379–410. [Google Scholar] [CrossRef] [Scilit]
- Chen, M.; Xu, Y.; Zhao, J.; Wei, X. Turing-Hopf Bifurcation Analysis in a Diffusive Ratio-Dependent Predator-Prey Model with Allee Effect and Predator Harvesting. Entropy 2023, 26, 18. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- She, G.; Yi, F. Stability and bifurcation analysis of a reaction-diffusion SIRS epidemic model with the general saturated incidence rate. J. Nonlinear Sci. 2024, 34, 101. [Google Scholar] [CrossRef] [Scilit]
- She, G.; Yi, F. Dynamics and bifurcations in a nondegenerate homogeneous diffusive SIR rabies model. SIAM J. Appl. Math. 2024, 84, 632–660. [Google Scholar] [CrossRef] [Scilit]
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.