


Abstract
This paper introduces a compact pneumatic artificial muscle (CPAM) that integrates a coaxial rod and an internal helical compression spring (stiffness 9750 N/m) into a McKibben-type outer muscle and compares it to a commercial DMSP-20-200N from FESTO Budapest, Hungary, with identical outer geometry and materials. Both actuators were mounted in a force-controlled test rig, pre-tensioned, and then cycled quasi-statically between their stretched and maximally contracted states at 13 internal pressures. For each pressure, median loading and unloading force–contraction curves were obtained from five repeats measuring both the cylinder excitation force and a load cell, and hysteresis was quantified by a normalized loop area based on peak force and common contraction range. Under the rated load of 2000 N at 0.6 MPa, the CPAM elongates less (−1.5% vs. −3%) and generates higher forces over most of the contraction range. The normalized hysteresis index of the CPAM is markedly lower at low pressures (≈0.05–0.25 MPa, reductions of about 10–25%), similar near 0.30 MPa, and slightly higher at 0.35–0.60 MPa (≈6–14%).
1. Introduction
Pneumatic artificial muscles (PAMs) are lightweight, compliant actuators that mimic several key properties of biological muscle, such as a monotonic force–contraction curve, a high force-to-weight ratio, and intrinsic compliance under load [1,2,3]. They have been deployed in biorobotics, rehabilitation devices, industrial manipulators and aerospace demonstrators, typically in antagonistic arrangements that exploit their muscle-like behavior for safe human–robot interaction [4,5,6]. In most of these applications, the actuator is a McKibben-type muscle: a rubber bladder surrounded by a braided sleeve and terminated in rigid end fittings.
The static behavior of McKibben muscles is often described by geometrical models that relate axial force F to internal pressure P and contraction ε. Starting from energy conservation, the muscle can be viewed as a pressure-driven “gas spring” where F ≈ −P·dV/dL, and the braid geometry leads to the classical Schulte, Chou–Hannaford and Tondu–Lopez formulas with parameters depending on the initial braid angle and radius [2,7,8,9]. These models are attractive because they are simple and, after empirical correction factors for end effects, approximate the static force–contraction–pressure characteristics of commercial muscles reasonably well [10,11,12]. Consequently, many application papers adopt some variant of these geometric models for actuator sizing and control design.
However, real PAMs depart from these idealized models in several important ways. Experimental studies consistently report reduced force compared to ideal predictions, significant hysteresis in the force–length relationship, threshold pressure effects, and temperature-dependent drift [2,13,14,15]. Detailed measurements show that the width of the tension–length loop is almost independent of speed over a wide range, indicating that hysteresis is dominated by dry (Coulomb) friction and viscoelastic effects rather than simple viscous damping [2,13]. Tondu and others have argued that hysteresis originates primarily from strand-on-strand friction in the braid and complex end-region deformation and that no single static model can simultaneously capture all these effects with high accuracy [2,13,16,17]. This friction- and geometry-induced hysteresis complicates accurate position and force control and motivates the development of phenomenological hysteresis models such as Maxwell-slip, Prandtl–Ishlinskii and related operators (standard scalar hysteresis operators) [18,19,20,21,22].
One way to reduce hysteresis and improve controllability is to modify the internal structure of the actuator. Pleated pneumatic muscles, which unfold pleats rather than stretching the membrane, exhibit very low hysteresis and negligible threshold pressure, enabling fast and precise motion with simple PI control [1,23,24]. Other designs introduce internal rods or compound architectures [5,25]. For example, double-acting sleeve muscles with a central solid rod can reduce air consumption relative to an identical muscle without a rod, at the cost of added mass and reduced extension capability. Bending and bidirectional PAMs use internal rods and frames to tailor stiffness, bending behavior and load capacity [5,25,26,27]. These studies collectively demonstrate that adding internal mechanical structure can substantially reshape the static and dynamic characteristics of PAMs.
At the same time, high-fidelity continuum-mechanics models for plain PAMs have become increasingly complex, combining thick-walled cylinder mechanics, advanced hyperelastic laws and Mullins softening to match experimental force–contraction data [10,28,29,30,31]. While such models can be accurate, their complexity and parameter sensitivity limit their usefulness for real-time control or design optimization. From a control and system-identification perspective, it is therefore appealing to explore actuator designs whose behavior is closer to an ideal spring or gas-spring element so that simpler models suffice.
In this work, we introduce and experimentally characterize a compact pneumatic artificial muscle (CPAM) that incorporates a coaxial rod and an internal mechanical spring inside a McKibben-type outer muscle. The CPAM shares the same outer geometry and materials as a commercial contraction muscle, so the primary difference between the two actuators is the internal spring–rod structure. The intuitive expectation is that the internal spring carries part of the load and linearizes the overall force–contraction behavior, while the rod constrains deformation, reduces end-region ballooning, and modifies the stress state in the braided sleeve [2,10,13,30]. If this architecture reduces the contribution of frictional and viscoelastic effects relative to the elastic backbone, the resulting actuator should exhibit smaller normalized hysteresis loops and more spring-like behavior. Reduced hysteresis, especially at low pressures, can improve positioning control in PAM-driven systems such as the ones used in [32] by decreasing history-dependent error and effective deadband between contraction and expansion paths.
Unlike spring-assisted PAM configurations that rely on external springs or linkages, the CPAM integrates the load-bearing elements within the actuator envelope, enabling a smaller footprint and simpler mechanical integration. In addition, the internal structure reduces the pneumatic volume, so less air mass is required to reach a given pressure, which may reduce pneumatic demand and improve responsiveness.
To investigate this hypothesis, we perform a side-by-side comparison between a commercial pneumatic artificial muscle and the proposed CPAM under identical boundary conditions. Both actuators are pre-stretched to a small initial strain, then cycled quasi-statically between this initial length and their maximum contraction at multiple internal pressures. For each pressure, we record force–contraction curves during loading and unloading and repeat the measurement multiple times to characterize variability. From these data, we extract the contraction range, blocked force, and a normalized hysteresis measure based on the loop area and peak elastic energy. By matching muscle length, diameter, materials, and operating pressures, we isolate the effect of the internal spring–rod on static performance and hysteresis. Note that temperature and humidity are not controlled variables in this experiment.
2. Materials and Methods
2.1. Actuators Under Test
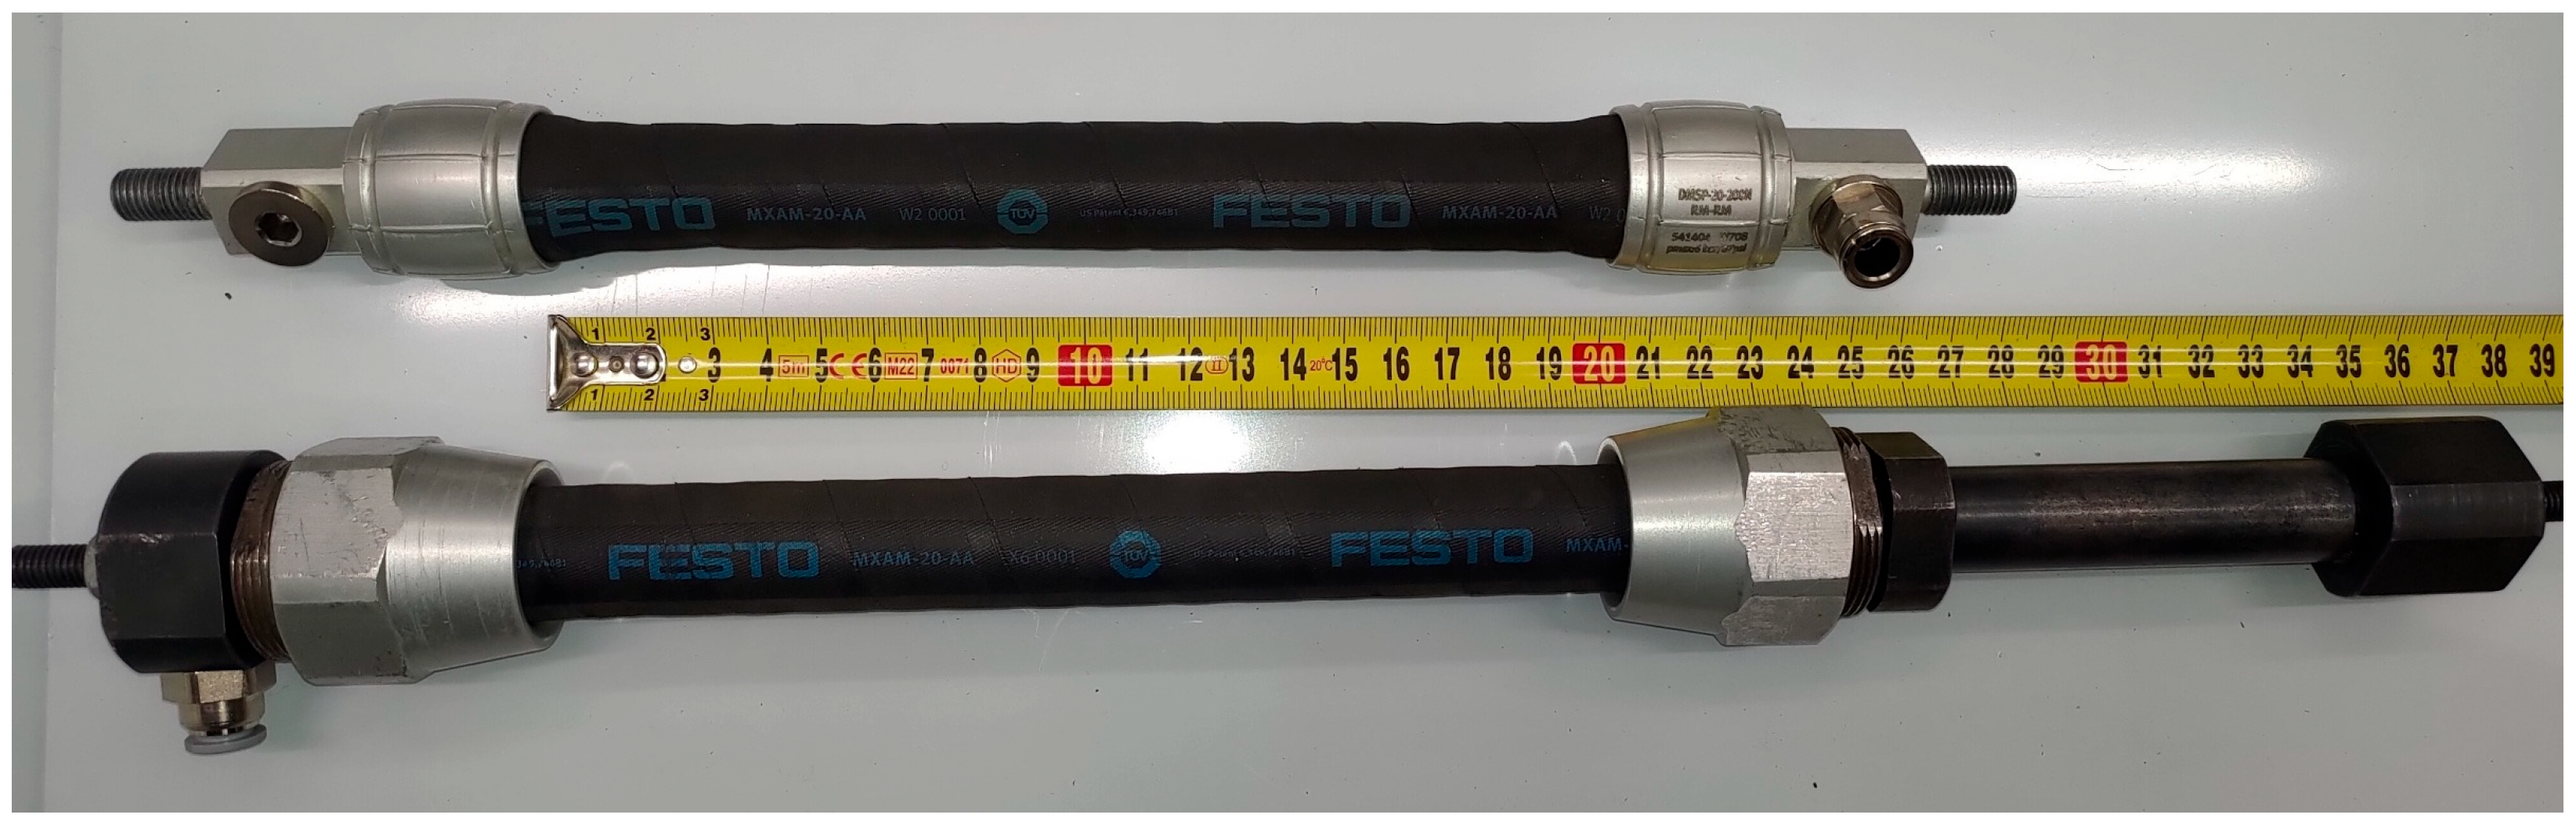
Two pneumatic artificial muscles (Figure 1) with identical outer geometry and materials were tested:
Figure 1.
PAM above and CPAM below.
- A commercial single-acting contraction PAM (type DMSP-20-200N, nominal diameter 20 mm, nominal length 200 mm)—Figure 2 shows the cross-section as seen in FESTO fluidic muscle catalog [33].
- A compact pneumatic artificial muscle (CPAM) developed in-house, using the same outer rubber bladder and braided sleeve, but incorporating a coaxial rod and an internal helical compression spring with a linear stiffness of 9750 N/m.
Figure 2.
Cross-section of PAM.
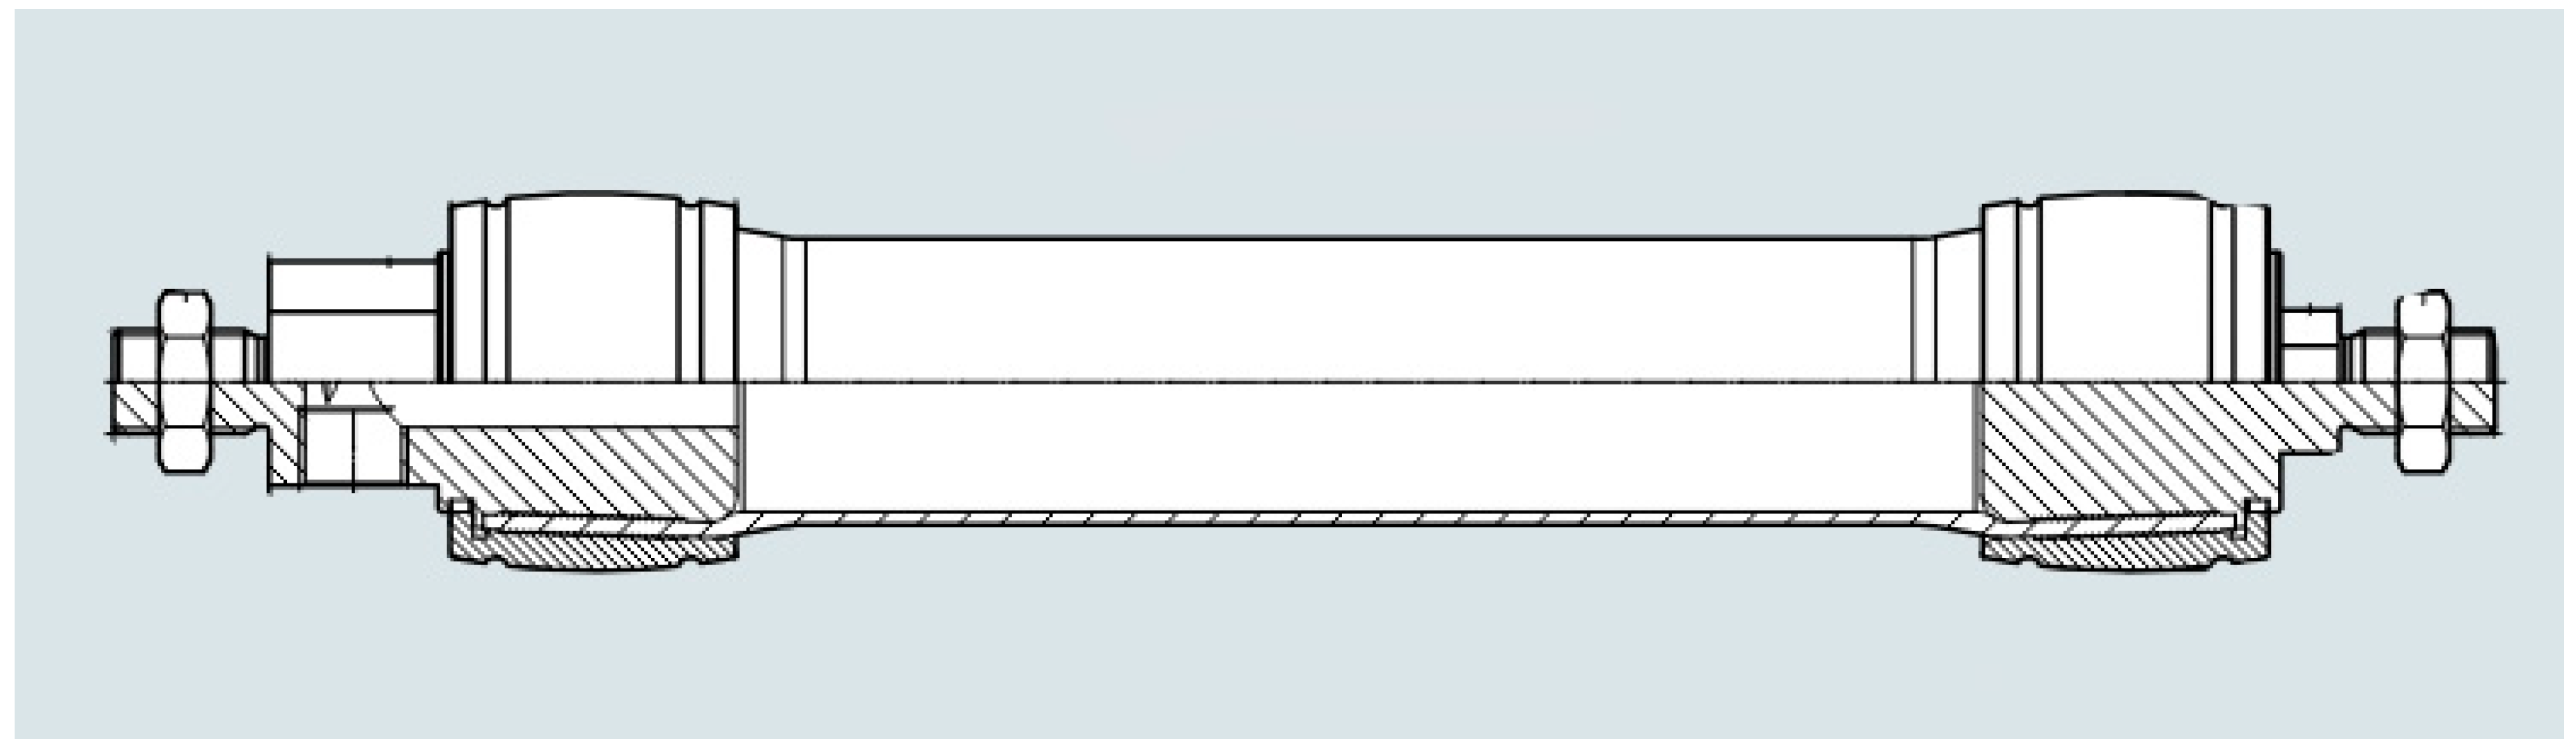
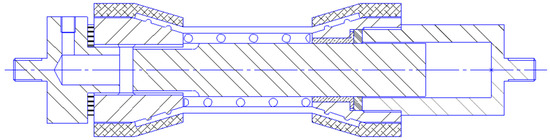
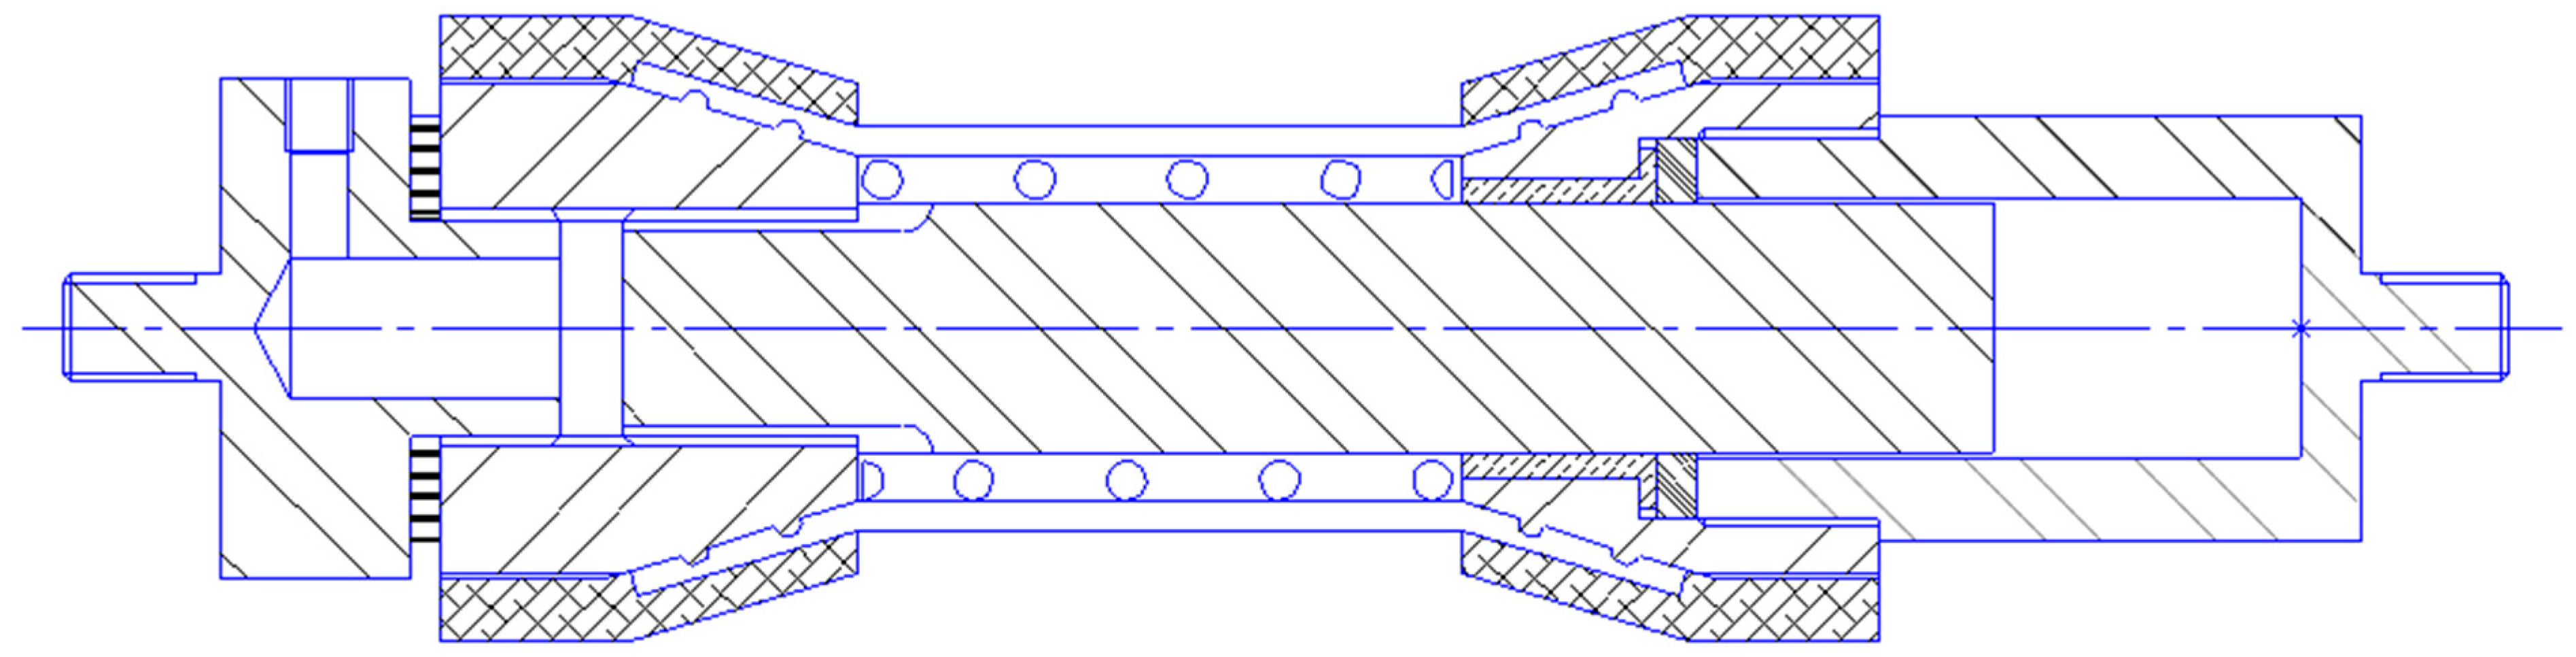
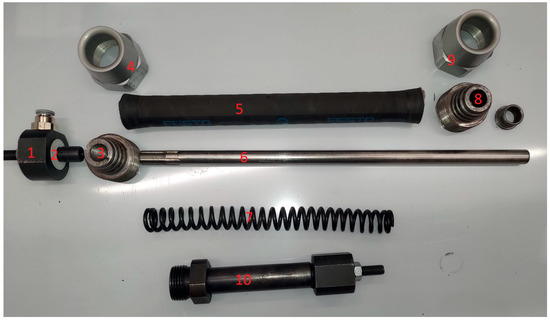
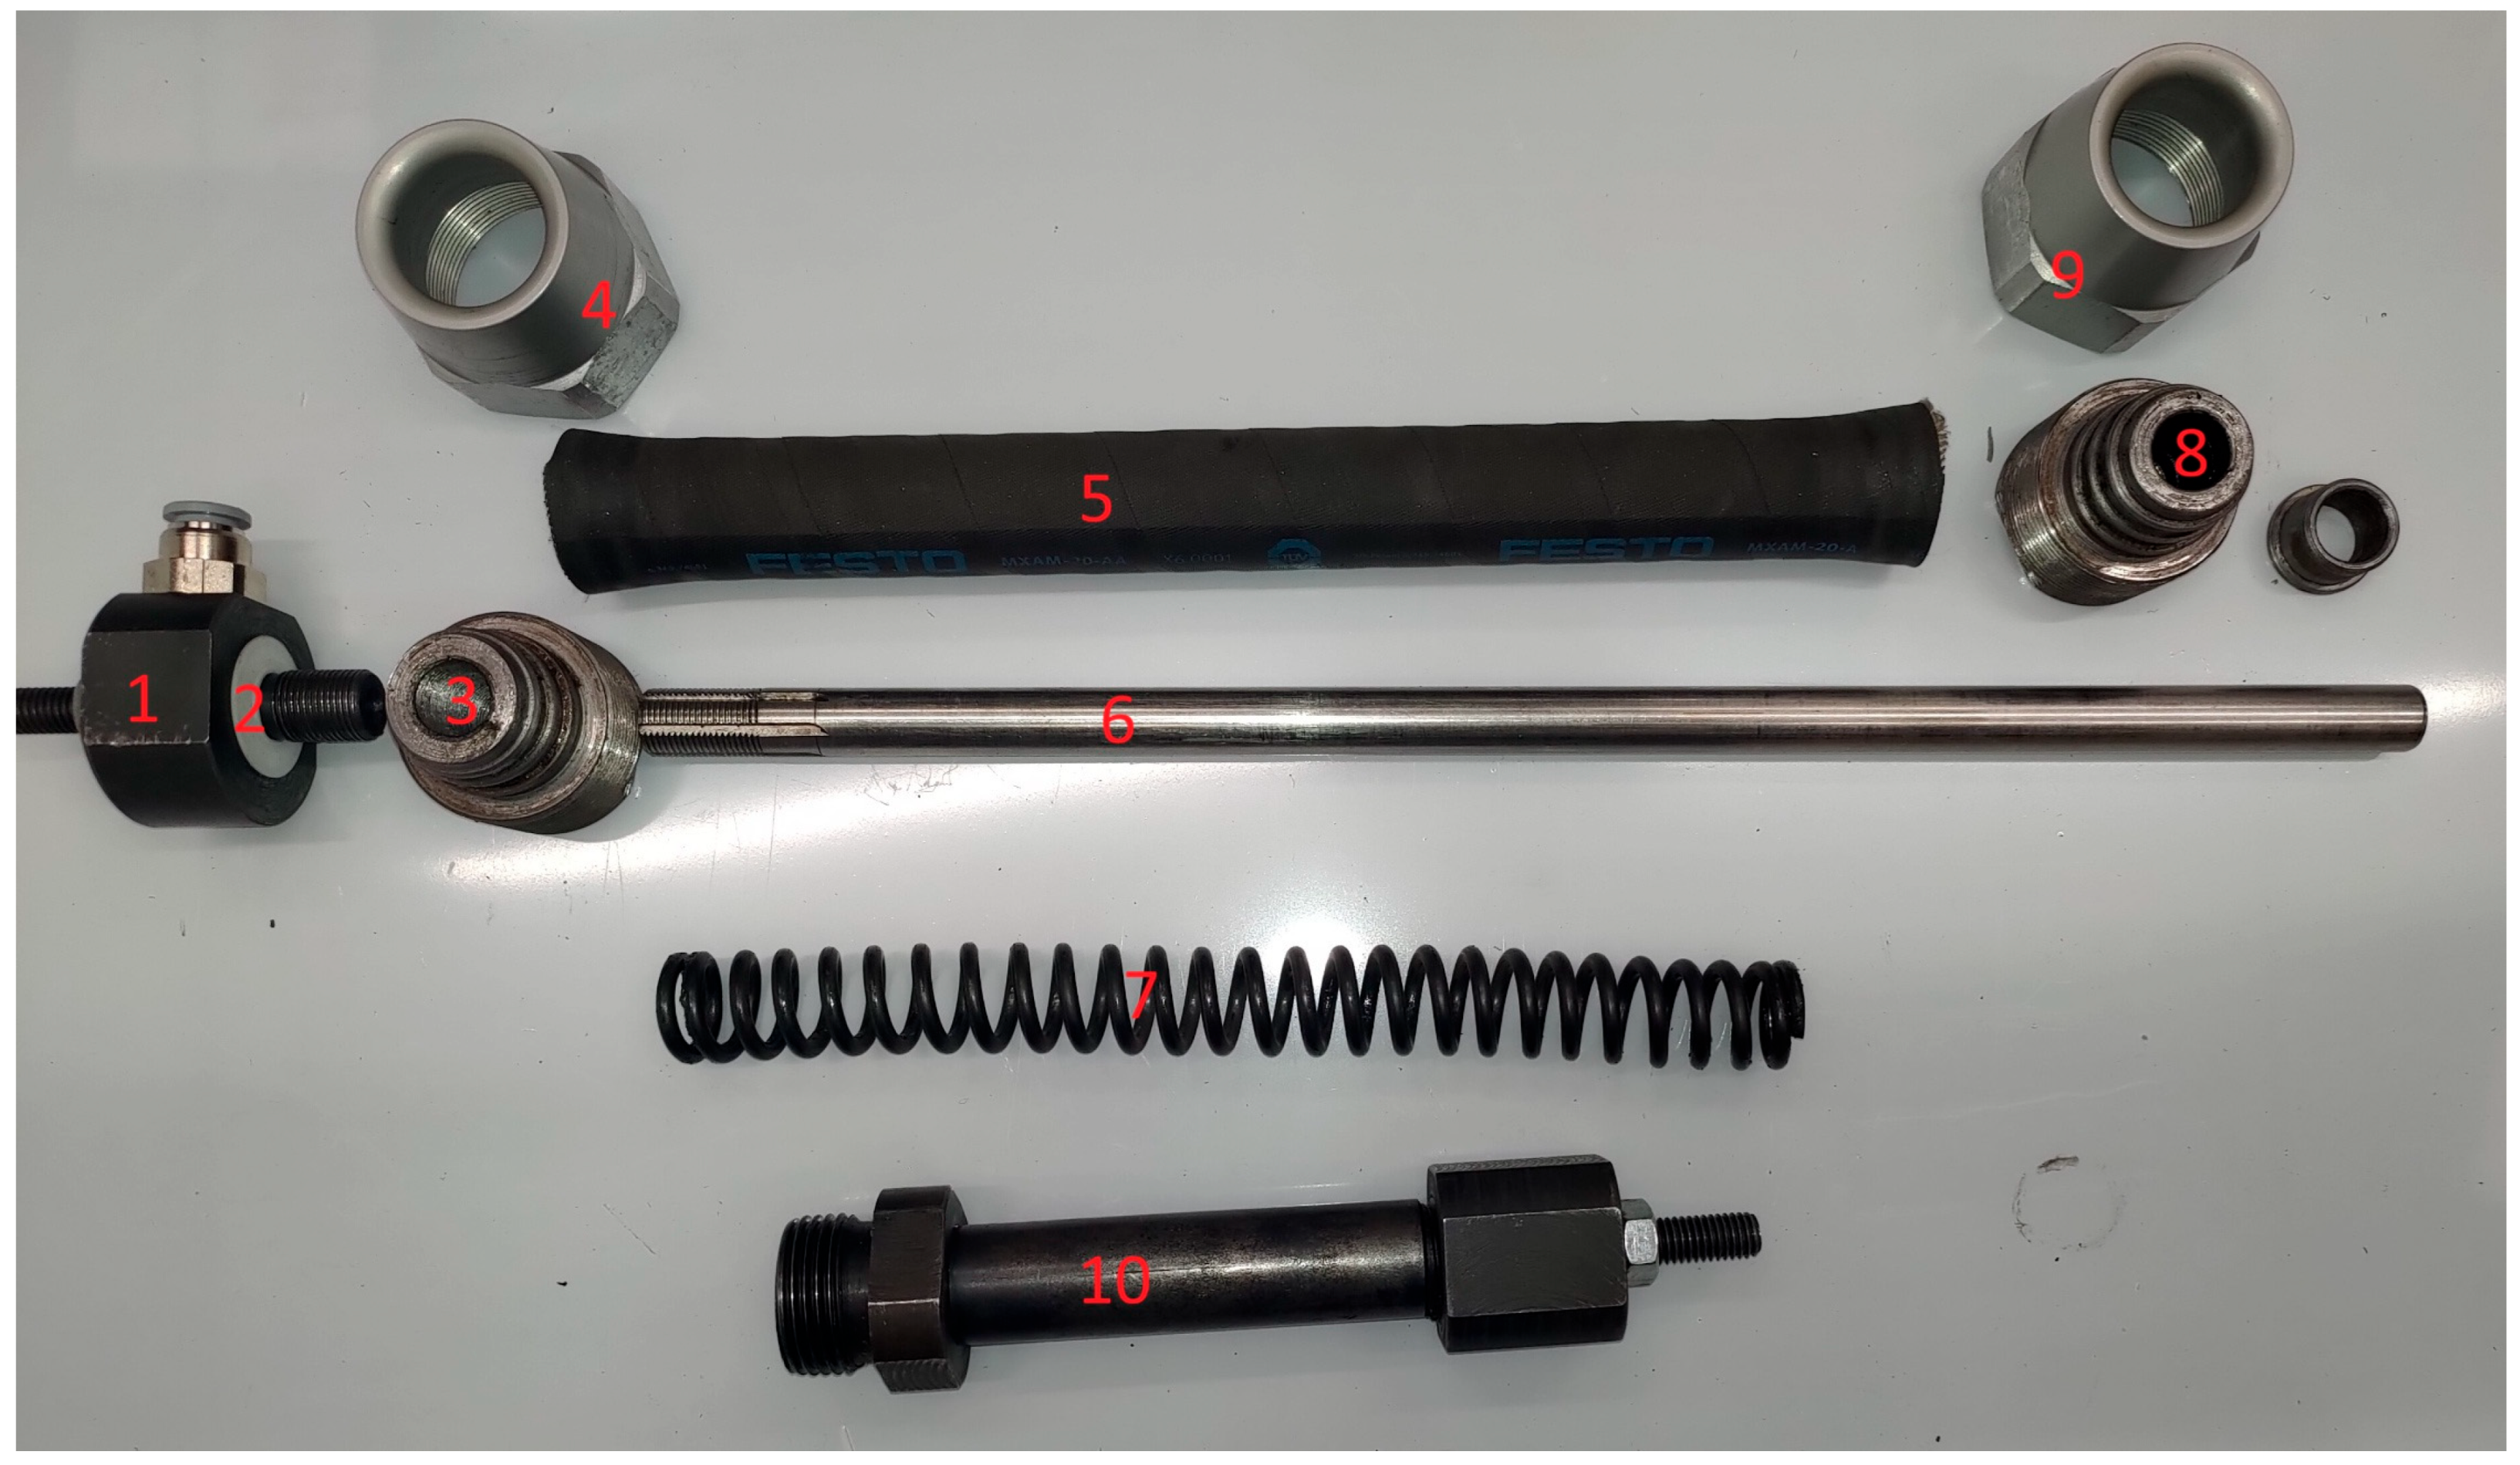
Figure 3 shows a schematic cross-section of the CPAM. The outer rubber membrane and braided sleeve are identical to the DMSP-20-200N. On the left side is an endcap (1), which provides a pneumatic connection to the muscle, as well as a threaded shaft to connect the CPAM to the load cell. The endcap is threaded into the left end fitting (3), and a Teflon ring (2) ensures an airtight connection. The left end fitting has a threaded outer surface on which a clamping nut (4) secures the rubber bladder and braided sleeve (5). On the right side of the left end fitting is the central rod (6) that runs along the actuator axis, and the compression spring (7) is mounted concentrically between the rod and the inner surface of the membrane. To allow air to pass into the muscle, the central rod has cutouts on its threaded end. The right end fitting (8) has the same threaded outer surface to which a clamping nut (9) secures the bladder and braided sleeve. Since the right end fitting needs to move along the central rod, a bronze bushing is used, and to make the end airtight, simmering is housed within the right end fitting. On the right side of the right end fitting is the right endcap (10), which keeps the simmering within the right end fitting. The right endcap also has a threaded shaft that allows connection to the cart. This internal structure constrains radial deformation of the membrane and provides an additional elastic load path in parallel with the pneumatic muscle. Figure 4 shows the disassembled CPAM with numbered references.
Figure 3.
Cross-section of CPAM.
Figure 4.
Disassembled CPAM.
Table 1 shows a brief overview comparing the two muscles under test.
Table 1.
Comparison of CPAM and DMSP-20-200 properties.
Both actuators were mounted at the same initial free length. The CPAM was assembled so that, at the pre-tensioned length used in the tests, the internal spring was already compressed and therefore contributes to the axial stiffness over the whole measured contraction range.
2.2. Experimental Setup
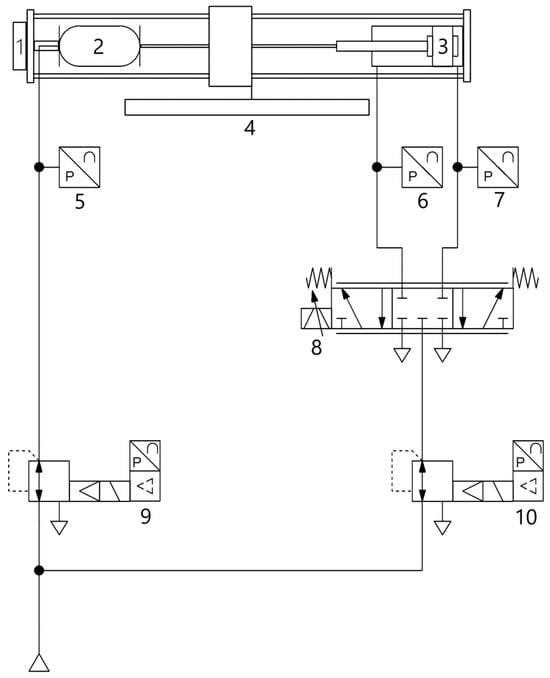
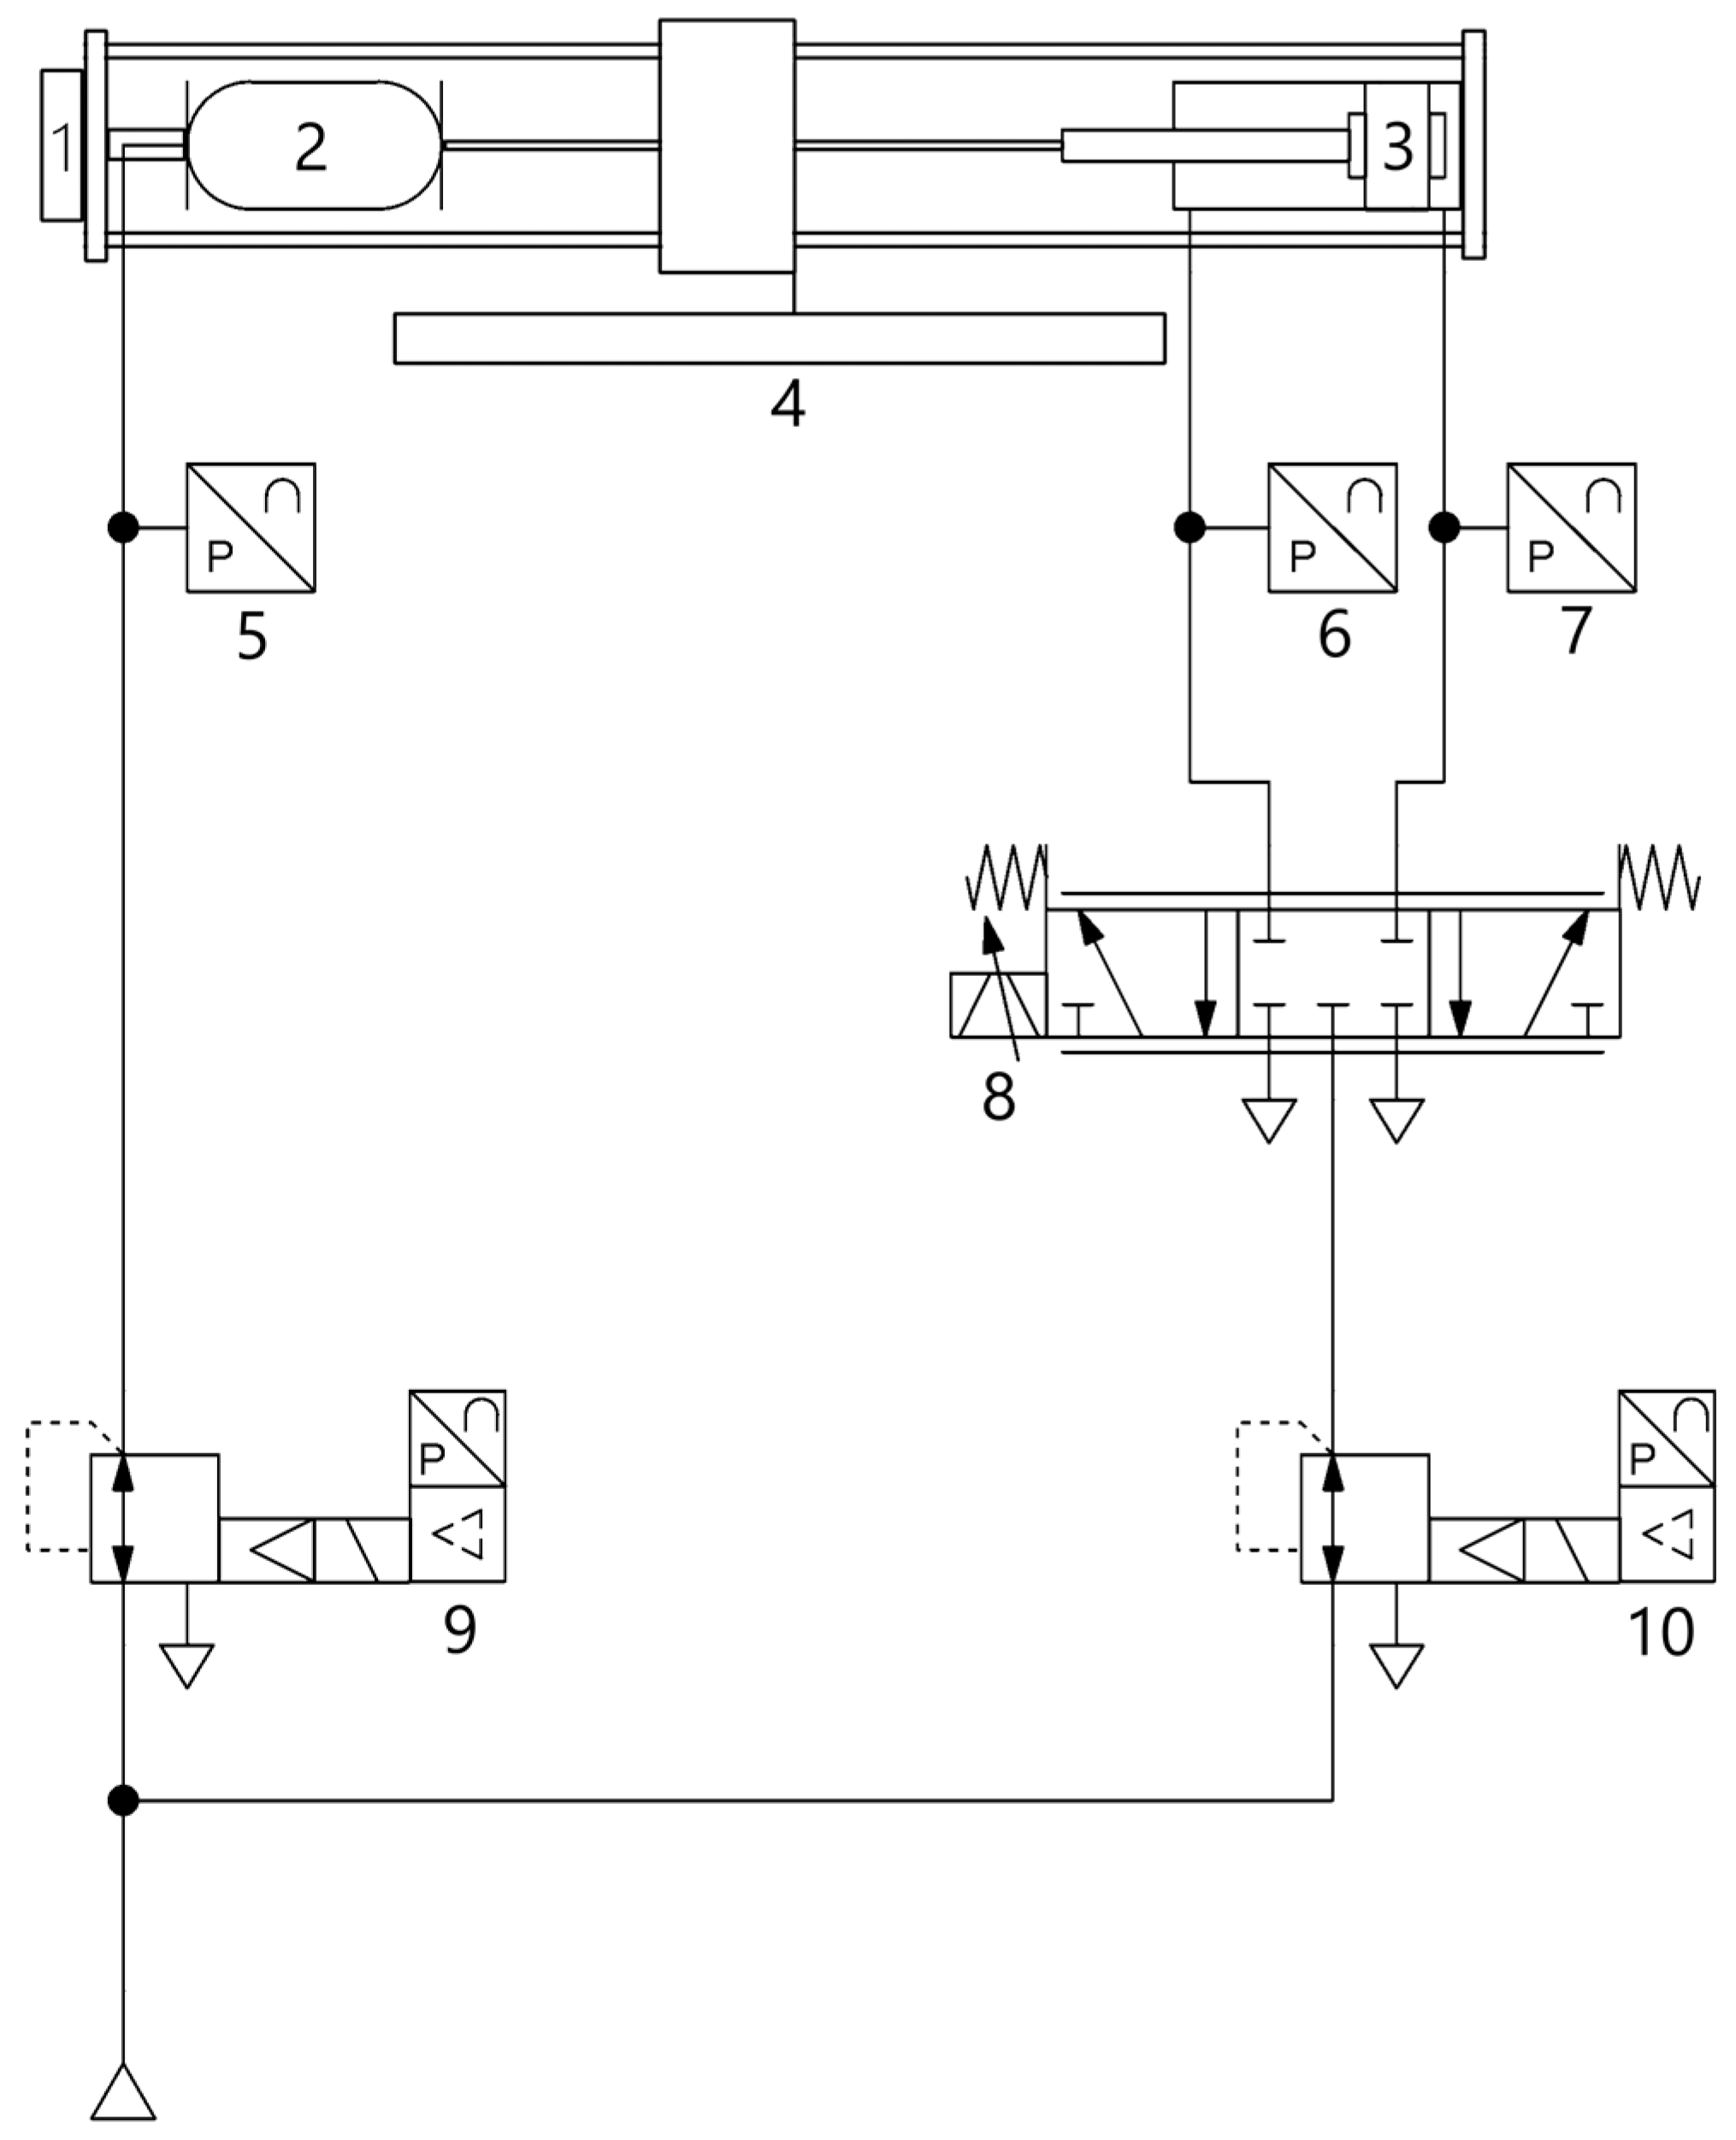
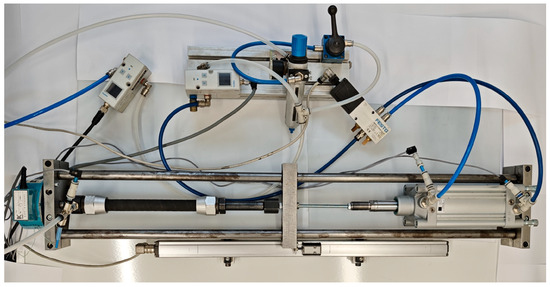
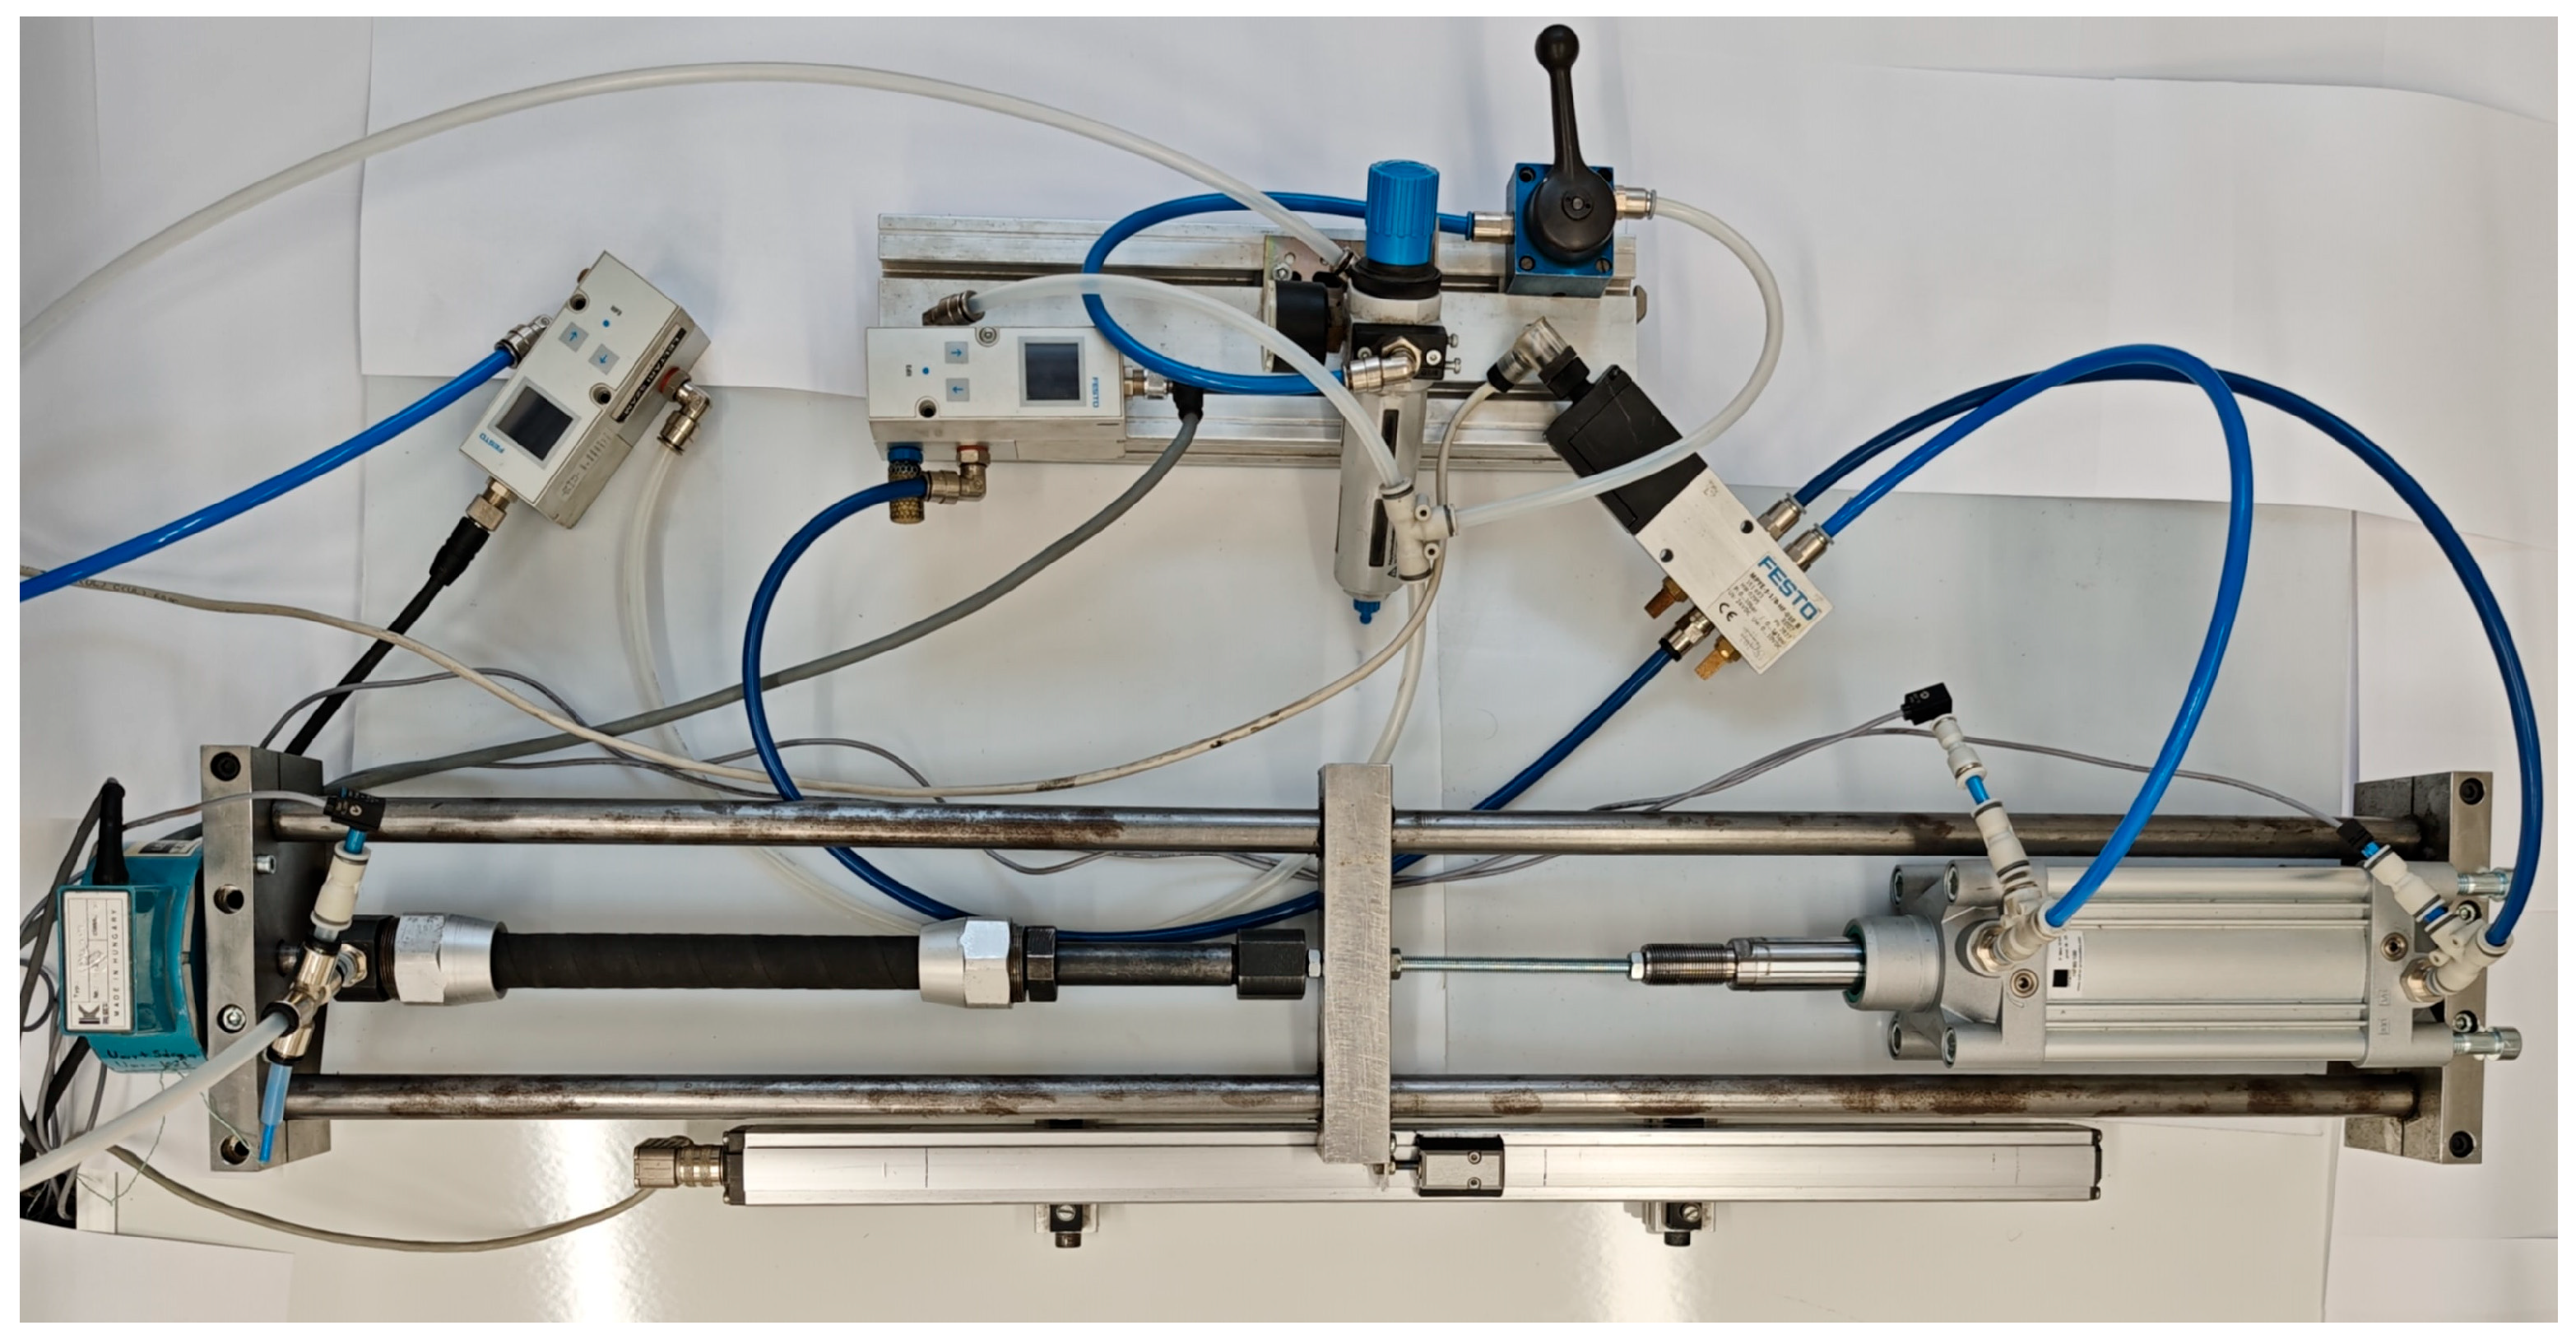
Figure 5 shows a schematic representation of the experimental rig, and Figure 6 shows a picture of the experimental rig.
Figure 5.
Schematic representation of experimental rig.
Figure 6.
Picture of experimental rig.
A double-acting pneumatic cylinder (type: HAFNER HIF80/100, Halászi, Hungary) (3) was used to apply a controlled excitation force to the muscle. Both cylinder ports, as well as the muscle being tested, were equipped with pressure sensors (type: FESTO SPTE-571484 B9, Budapest, Hungary) (5, 6, 7), and the cylinder was supplied via an electro-pneumatic pressure regulator (type: FESTO VPPM-6L-L1-G18-0l6H-V1N-S1C1, Budapest, Hungary) (10) driven by an analog control signal. By commanding the regulator output and the proportional valve (type: FESTO MPYE-5-1/8-HF-010 B, Budapest, Hungary) (8), a prescribed net force was generated at the piston–rod interface.
The cylinder rod was rigidly connected to a cart mounted on linear guide rails, such that the piston, cart, muscle (2) and load cell (type: KALIBER 8923-200kg, Budapest, Hungary) (1) all align along a single axis. This arrangement minimizes side loads and bending moments on both the muscle and the load cell. To process the signal of the load cell, a ClipX BM40 (Gottingen, Germany) was used.
On the opposite side of the cart, the test muscle (commercial PAM or CPAM) was mounted in series with a uniaxial load cell that measured the axial muscle force. The pressure of the muscle can be independently controlled with a pressure regulator (type: FESTO VPPM-6L-L-1-G18-0L6H-V1N-S1C1, Budapest, Hungary) (9). The far end of the load cell was fixed to the stationary frame of the rig. Muscle length (or equivalently, contraction percentage) was determined from the cart position using a linear position sensor (type: BALLUF BTL5-S101-M0500-P-S32, Veszprém, Hungary) (4) referenced to the fixed frame.
All analog signals (two chamber pressures, muscle pressure, load–cell force, cart position, and the regulator command) were acquired synchronously using a real-time data acquisition system with a sampling frequency of 3 ms. The data acquisition was performed with a National Instruments CRIO-9040 (Debrecen, Hungary) with the following modules: NI 9474, NI 9201, and NI 9263. For each operating point, data were recorded on the cycle the position reached the set position ±15 microns.
The excitation force produced by the pneumatic cylinder was calculated from the measured chamber pressures and the piston areas. Let Ppos and Pneg denote the absolute pressures in the cap-end and rod-end chambers, respectively, and let Apos and Aneg be the corresponding effective piston areas (with Aneg = Apiston − Arod on the rod side). The net axial force exerted by the cylinder on the cart was then computed as shown in Equation (1):
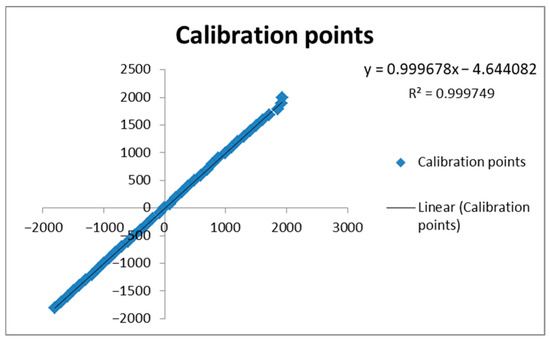
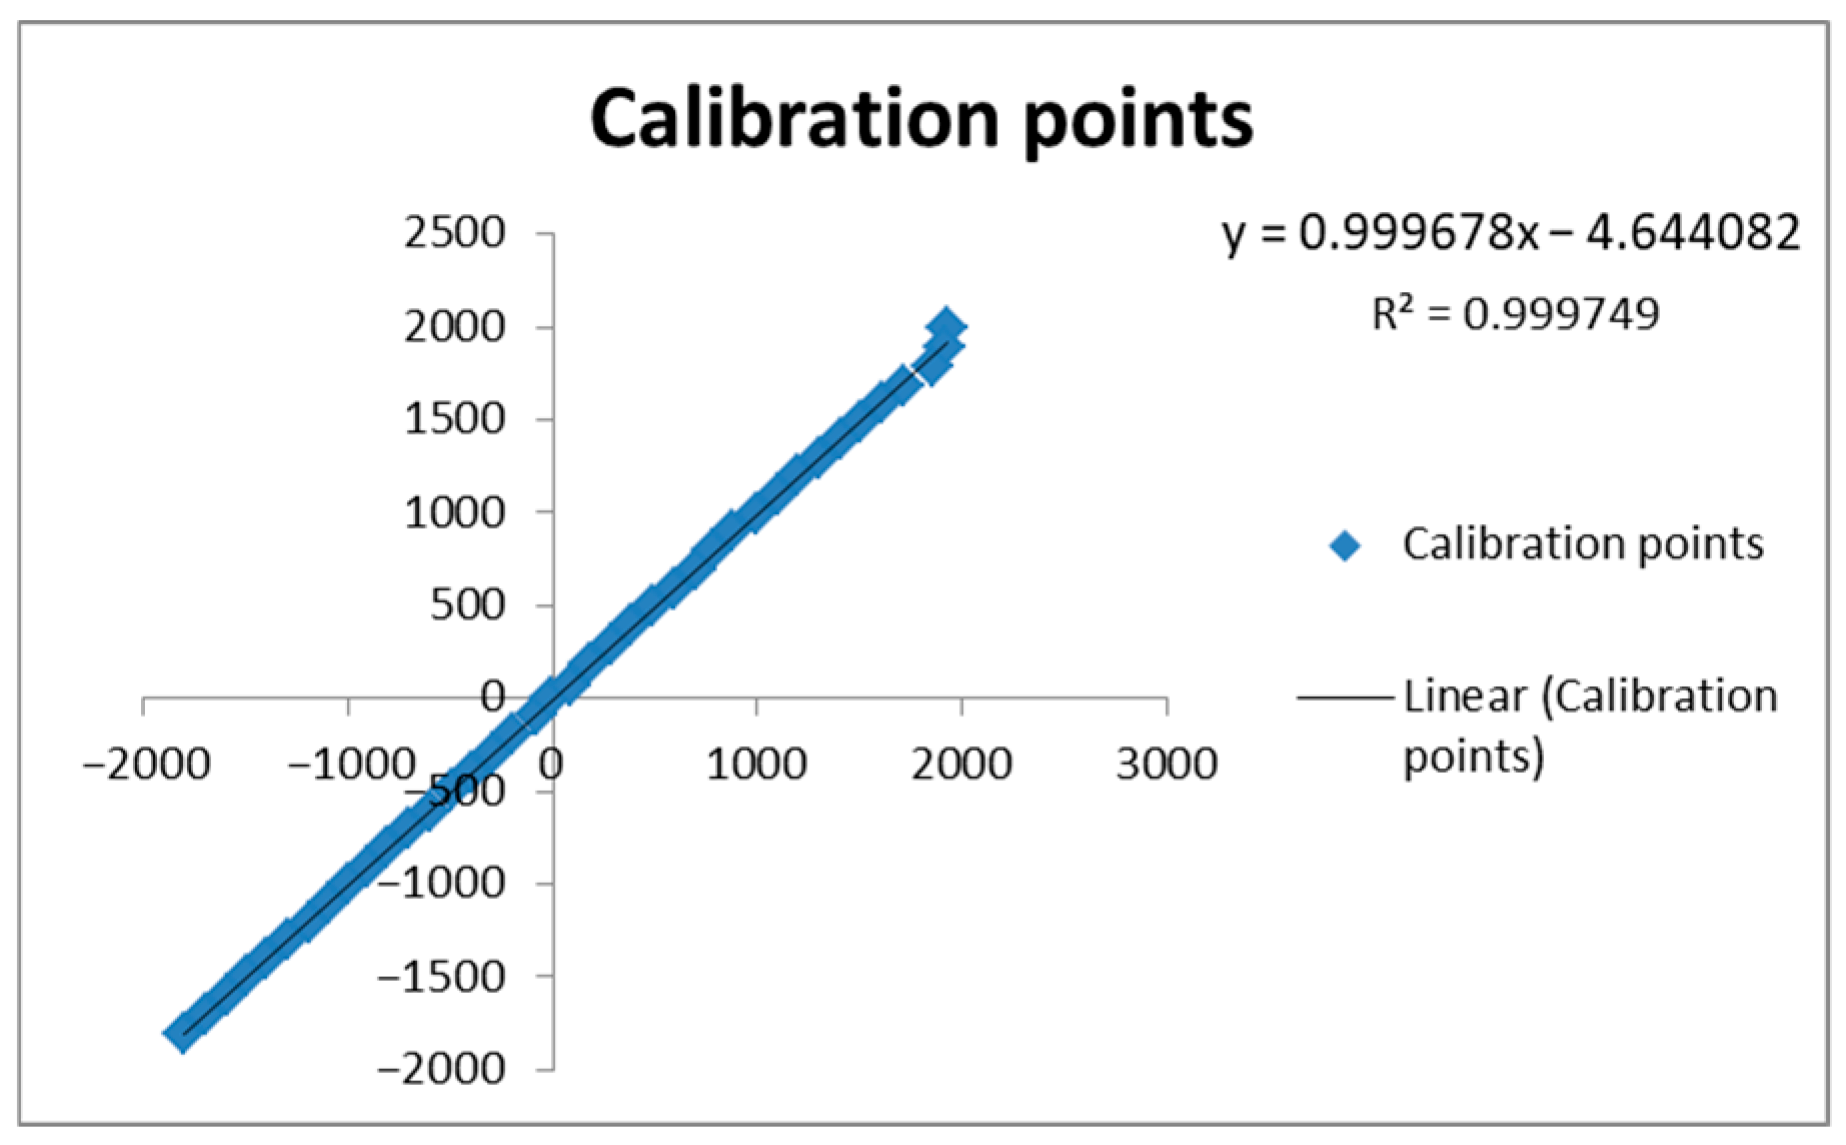
Before testing the muscles, the load cell was statically calibrated against Fexcitation. For calibration, the muscle was removed, and the cart was connected directly to the load cell through a rigid steel rod. Static force levels were generated by setting the regulator command such that Fexcitation took prescribed values between +2000 N and −1800 N. At each level, the load–cell output was recorded, and a linear calibration curve was fitted so that the calibrated load–cell reading Fmeasured matched Fexcitation over this range. The calibration curve can be seen in Figure 7. Table 2 shows a summary of the sensors used and their uncertainty.
Figure 7.
Calibration of load cell and excitation force.
Table 2.
Instrumentation and uncertainty summary.
During muscle tests, both Fexcitation(t) and Fmeasured(t) were recorded simultaneously. This allows us to distinguish between input-side behavior (force applied by the pneumatic system) and output-side behavior (force transmitted through the muscle).
2.3. Pre-Tensioning, Test Protocol and Data Selection
Before the hysteresis measurements, both muscles were first characterized under the maximum operating conditions specified by the manufacturer. The cylinder was commanded to apply a pulling force of 2000 N at an internal pressure of 0.6 MPa, which corresponds to the upper limits in the DMSP-20-200N data sheet. Under this combined loading, the commercial muscle stretched to a maximum of approximately −3% relative to its free length at atmospheric pressure, whereas the CPAM stretched only to about −1.5%. This difference is attributed to the internal spring and rod in the CPAM: the spring has approximately the same diameter as the rubber membrane when at rest. When stretched, the membrane cannot bow inward as in the commercial muscle, leading to a stiffer tensile response in extension.
For the quasi-static hysteresis tests, each actuator (commercial PAM and CPAM) was then tested at 13 discrete pressure setpoints from 0 to 0.6 MPa in 0.05 MPa increments to cover the full rated range. At the beginning of each measurement sequence, the corresponding muscle was brought close to its maximum stretched state (about −3% for the DMSP-20-200N and −1.5% for the CPAM) and held there for 10 s. This pre-tensioning step was used as a conditioning cycle to stabilize the braid and bladder configuration and to reduce short-term history effects from preceding cycles. After the dwell, the force ramp for the actual measurement was initiated.
For each pressure level, the following procedure was applied:
- Pressure for the muscle was set to a specified level.
- Excitation force was set so the muscle was at its pre-tensioned stretched state (−3% for the DMSP-20-200N, −1.5% for the CPAM). Force was held for 10 s.
- Quasi-static unloading (contraction branch). Starting from this stretched length, the net excitation force Fexcitation was ramped at a constant rate of approximately −4 N/s, such that the cart moved slowly and dynamic effects remained negligible. The ramp was discretized into 31 setpoints spanning the full contraction range from the stretched state to the maximum achievable contraction at that pressure.
- Quasi-static loading (expansion branch). After reaching maximum contraction, the process was reversed: Fexcitation was increased linearly at a rate of 4 N/s back towards the pre-tensioned state, again sampling 31 setpoints along the unloading path.
- Repetition. Steps 2–4 were repeated five times for each pressure level and each muscle.
Due to the way the force ramp was initiated after the pre-tensioning dwell, the first recorded force–contraction point after the stretched state typically occurred at a contraction slightly beyond the nominal pre-tension level and did not satisfy the prescribed quasi-static ramp condition of about 4 N/s. To ensure that the hysteresis analysis used only points obtained under a well-defined and uniform unloading/loading protocol, this first point was excluded when computing loop areas and normalized hysteresis indices. All remaining points were acquired while the excitation force was varied at exitation ≈ 4 N/s and were therefore used in the construction of the loading and unloading branches.
2.4. Data Processing and Hysteresis Quantification
Contraction ε was expressed as a percentage relative to the pre-tensioned length of the muscle. For each pressure level, the five repeats were resampled onto a common contraction grid over the contraction interval shared by the loading and unloading branches. Median loading and unloading curves were then computed for both the excitation force and the measured muscle force.
For a given muscle, pressure level and force signal, the hysteresis area A was defined as the area enclosed by the force–contraction loop. Numerically, A was approximated by trapezoidal integration of the closed loading–unloading path, as presented in Equation (2):
where the area under the expansion or contraction curve can be approximated as seen in Equation (3):
To compare hysteresis between muscles and pressures, a normalized hysteresis index HI was defined, as seen in Equation (4):
where Fmax is the maximum force reached on the loop at that pressure and Δε is the length of the contraction interval used for comparison at that pressure.
In addition to HI, the blocked force, maximum contraction, and cycle-to-cycle variability (coefficient of variation in loop area across the five repeats) were extracted for each pressure and each muscle. To quantify repeatability, HI was computed separately for each of the five cycles at a given pressure. The reported HI values are shown as the sample mean, together with a 95% confidence interval (CI95%) across the five cycles, computed using Student’s t distribution (n = 5), as shown in Equation (5):
where HImean is the mean across cycles for one set pressure, and sHI is the sample’s standard deviation.
3. Results
3.1. Maximum Stretch Under Rated Load
As a first comparison, both muscles were tested under the maximum operating conditions specified in the data sheet of the commercial actuator. The cylinder was commanded to apply a pulling force of 2000 N at an internal pressure of 0.6 MPa. Under this combined loading, the commercial DMSP-20-200N muscle elongated to approximately −3% relative to its free length at atmospheric pressure, whereas the CPAM elongated only to about −1.5%.
This reduced stretch under the same rated load is consistent with the presence of the internal spring and rod in the CPAM. Because the spring closely matches the diameter of the rubber membrane when the muscle is stretched, the membrane cannot bow inward as in the commercial muscle. As a result, the CPAM exhibits a higher tensile stiffness in extension. This difference in extension behavior sets the initial condition for the subsequent quasi-static contraction tests.
3.2. Contraction Range and Unloading (Contraction) Behavior
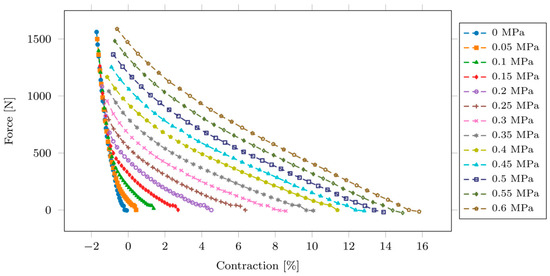
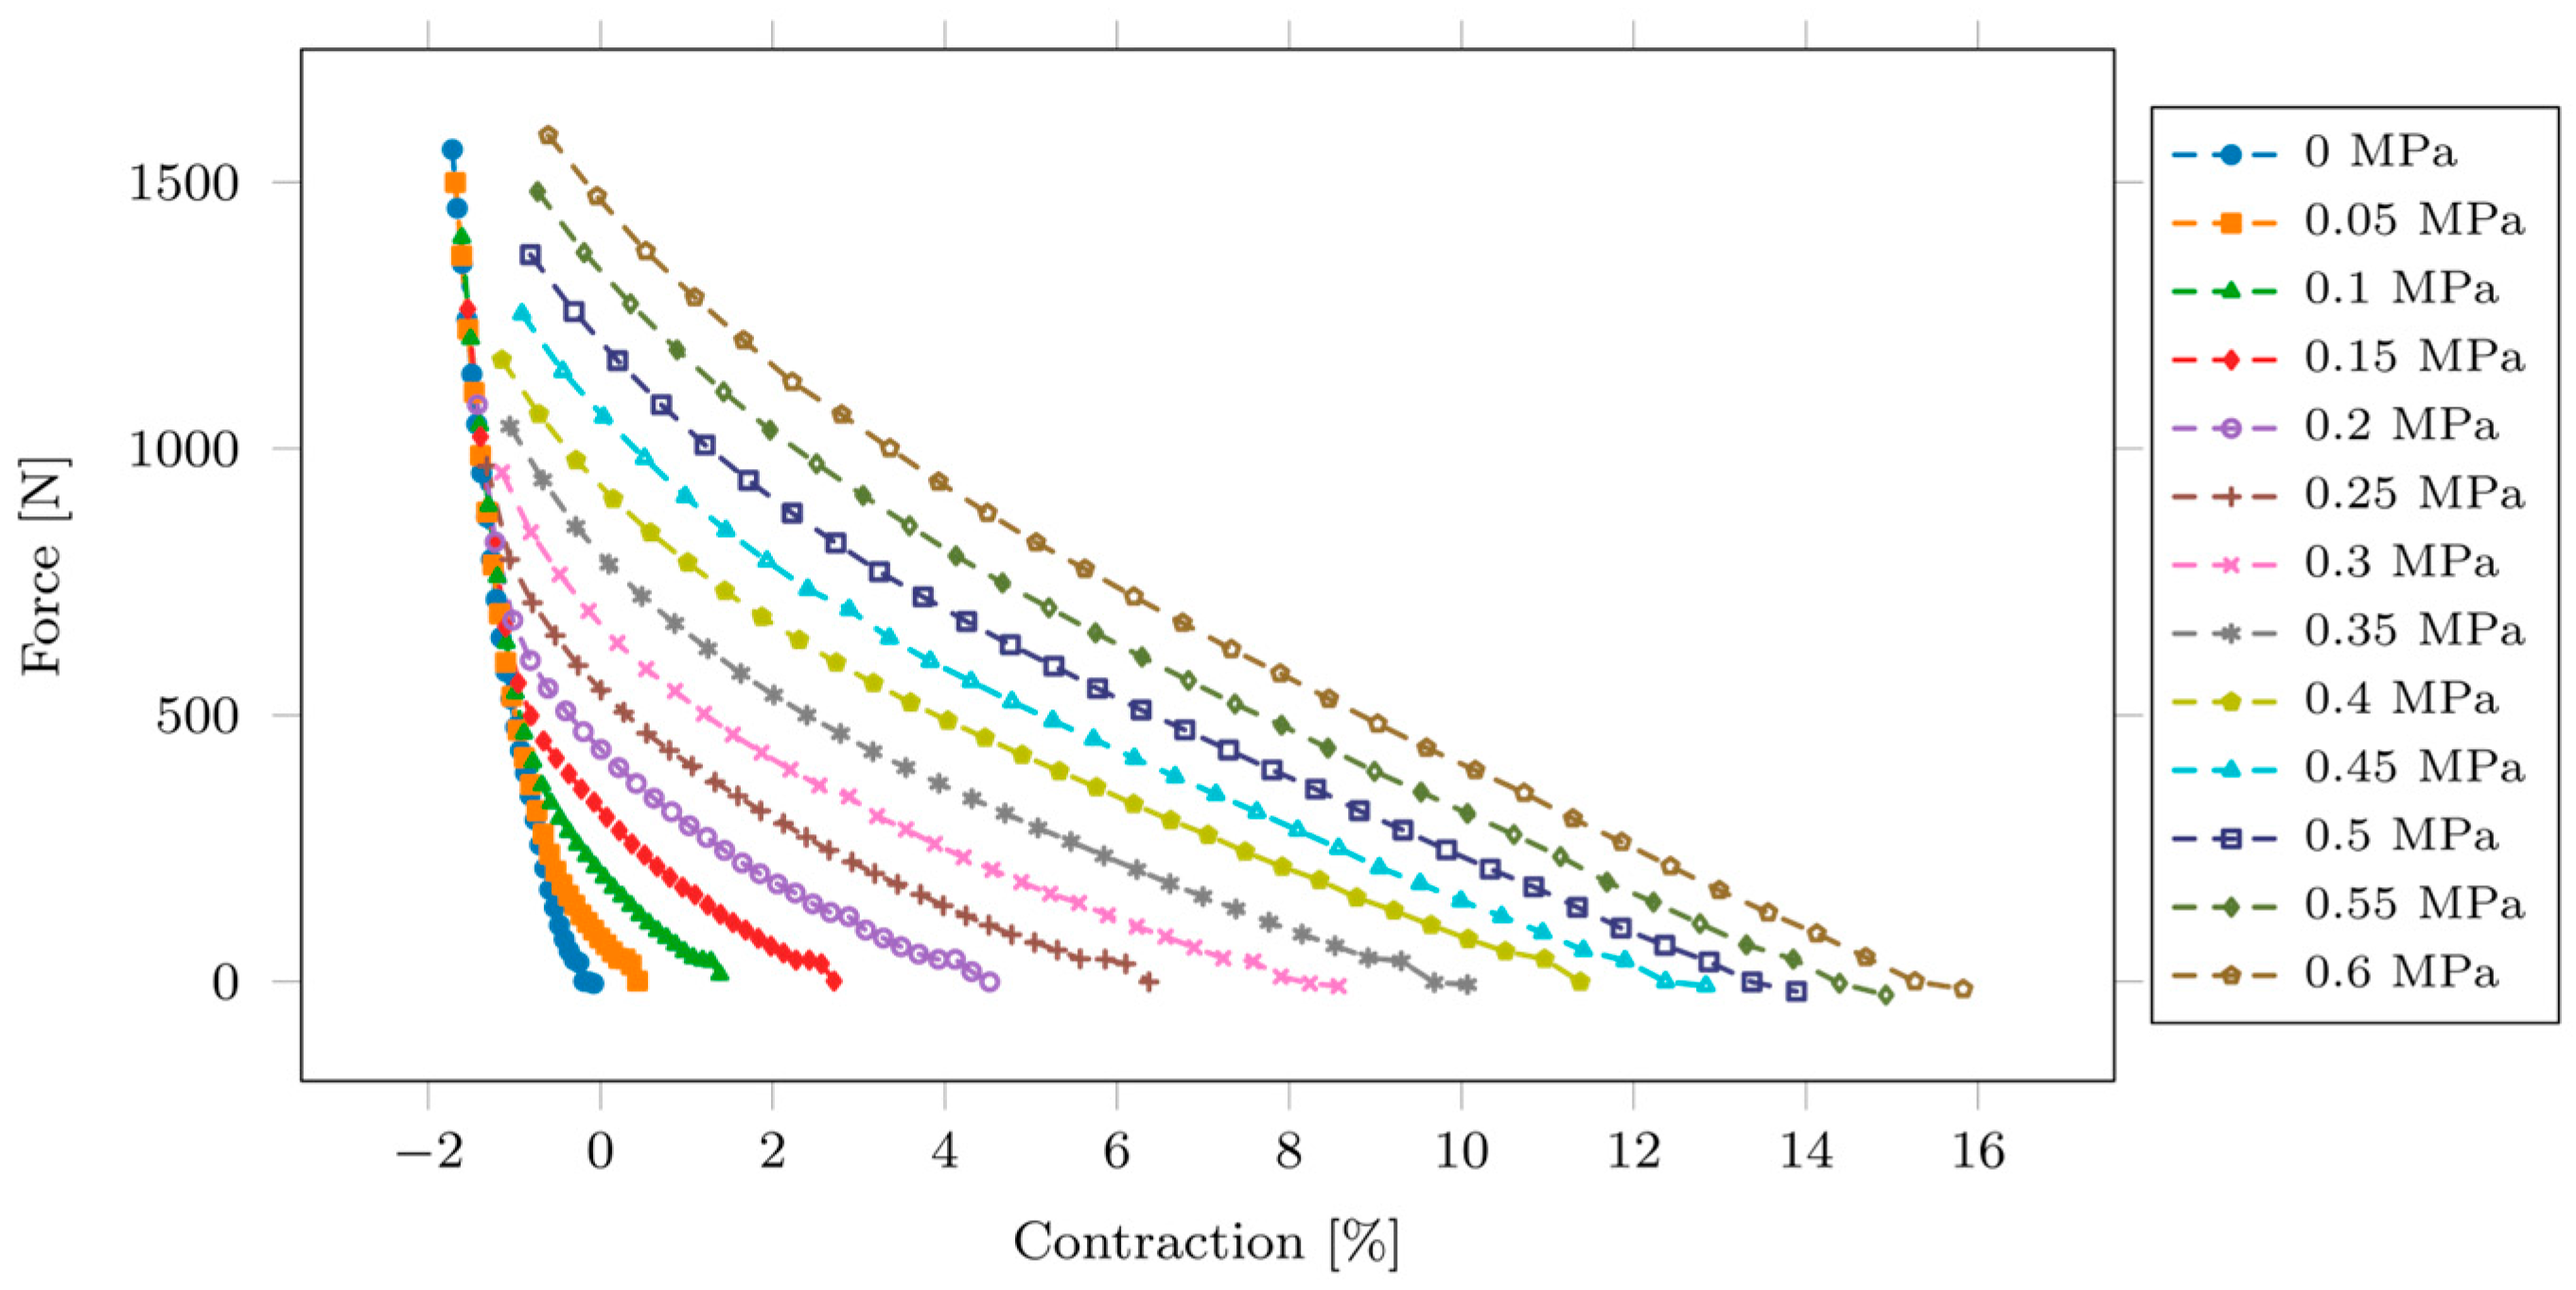
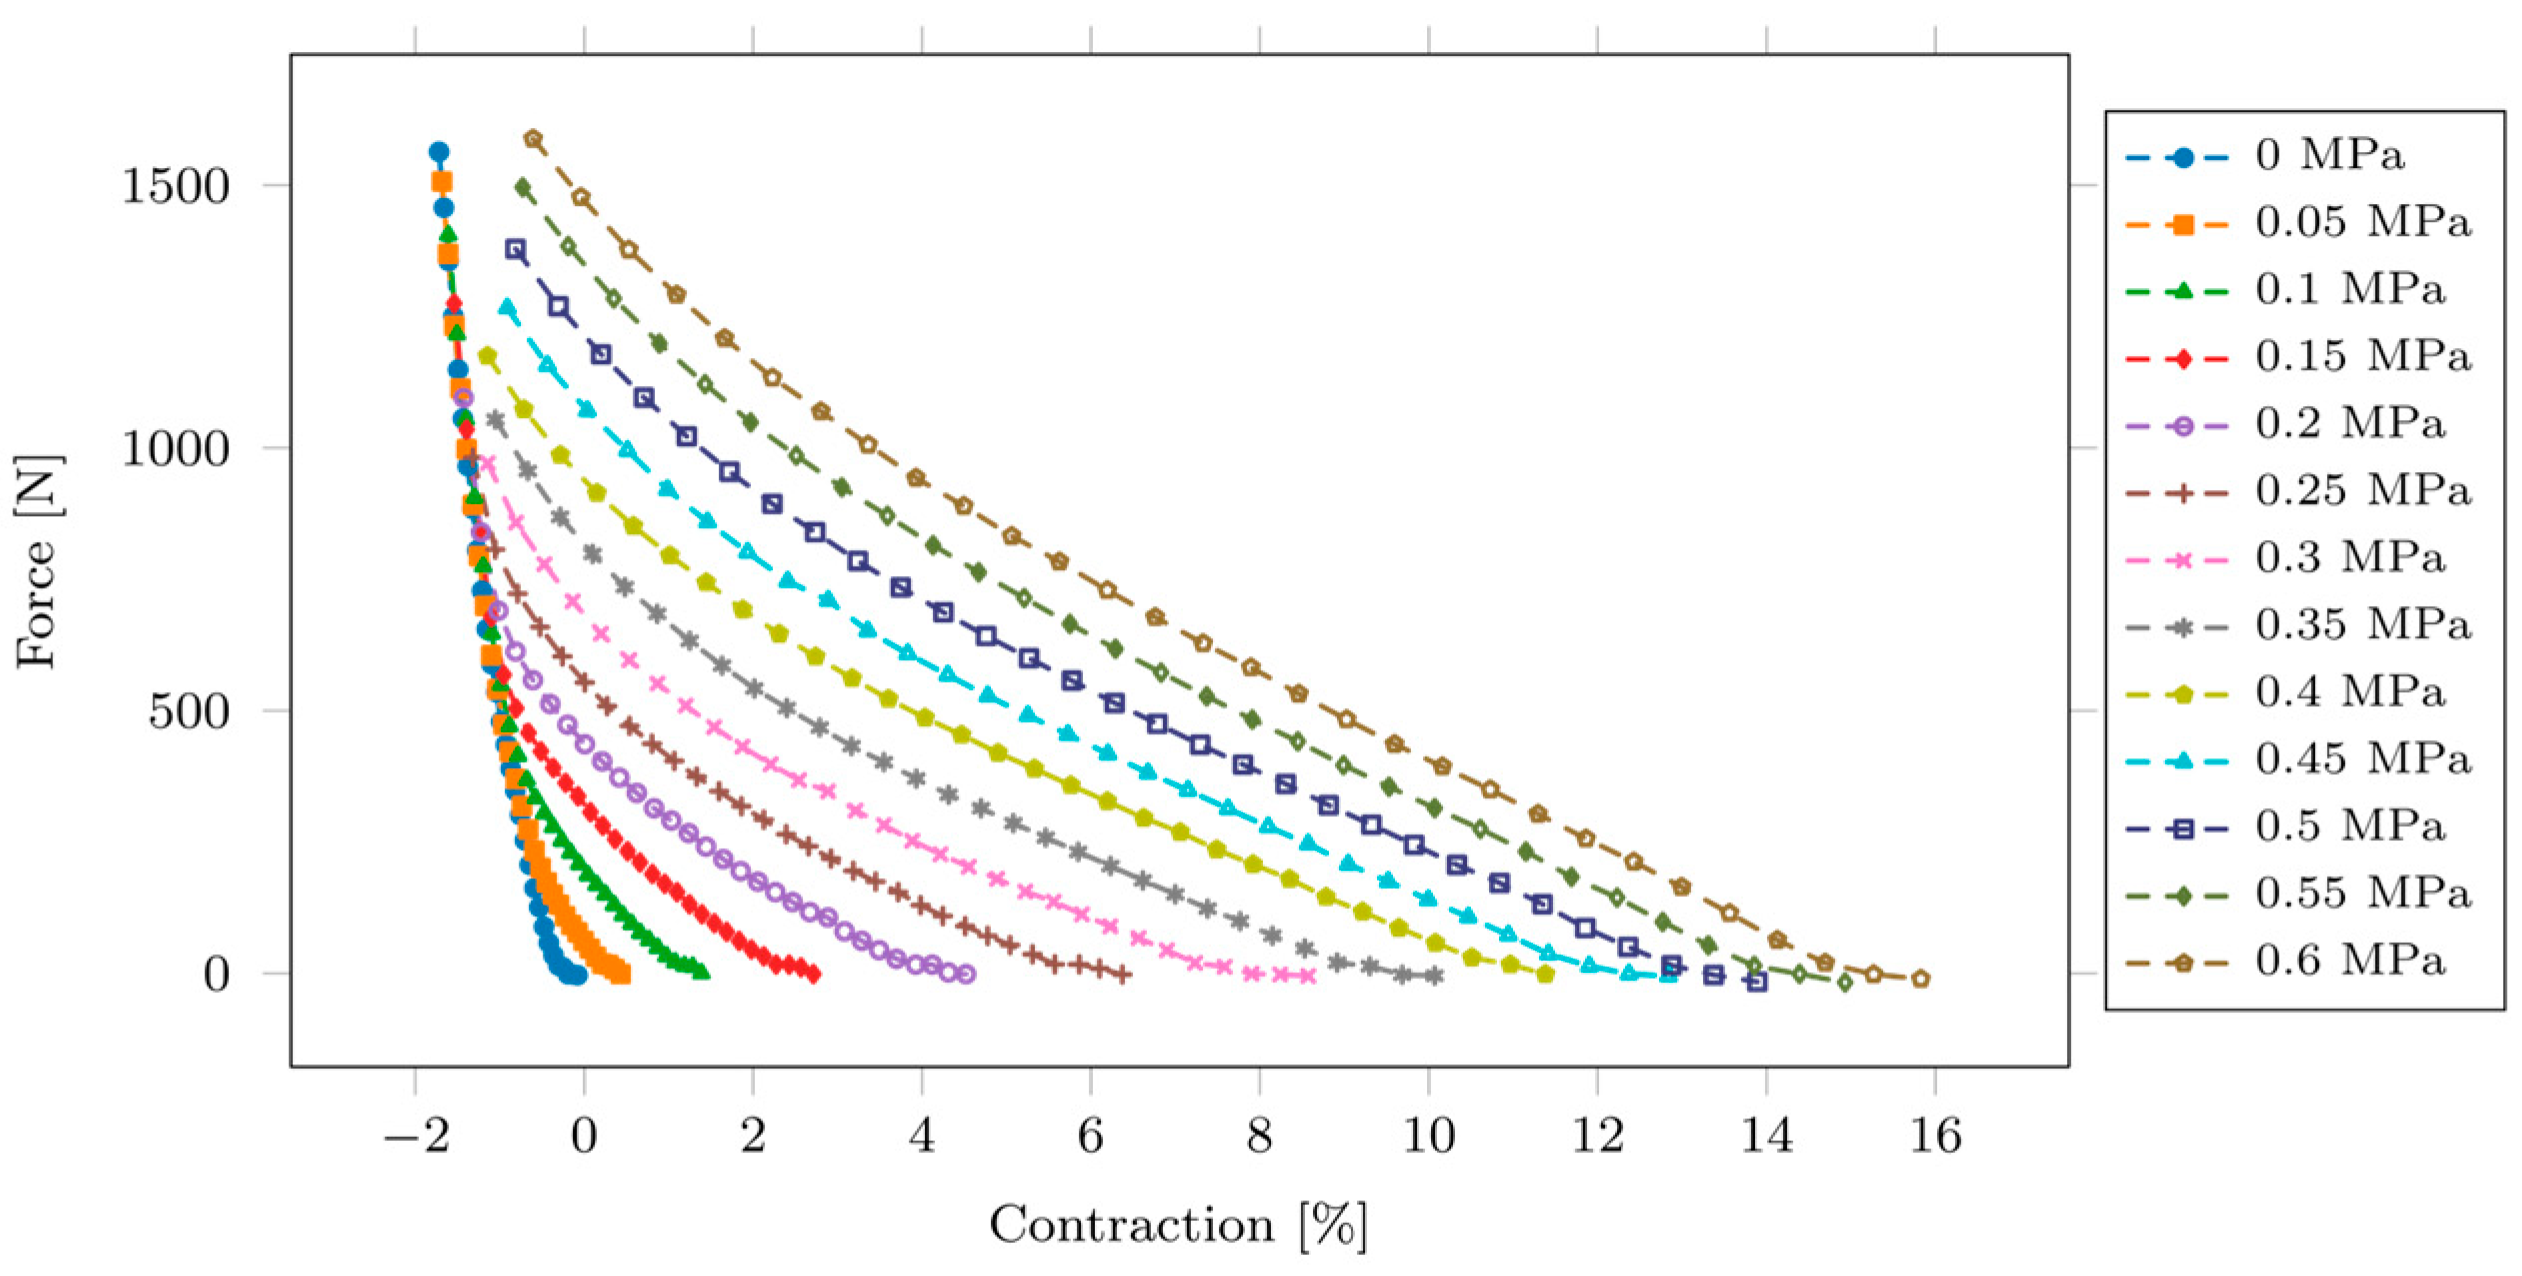
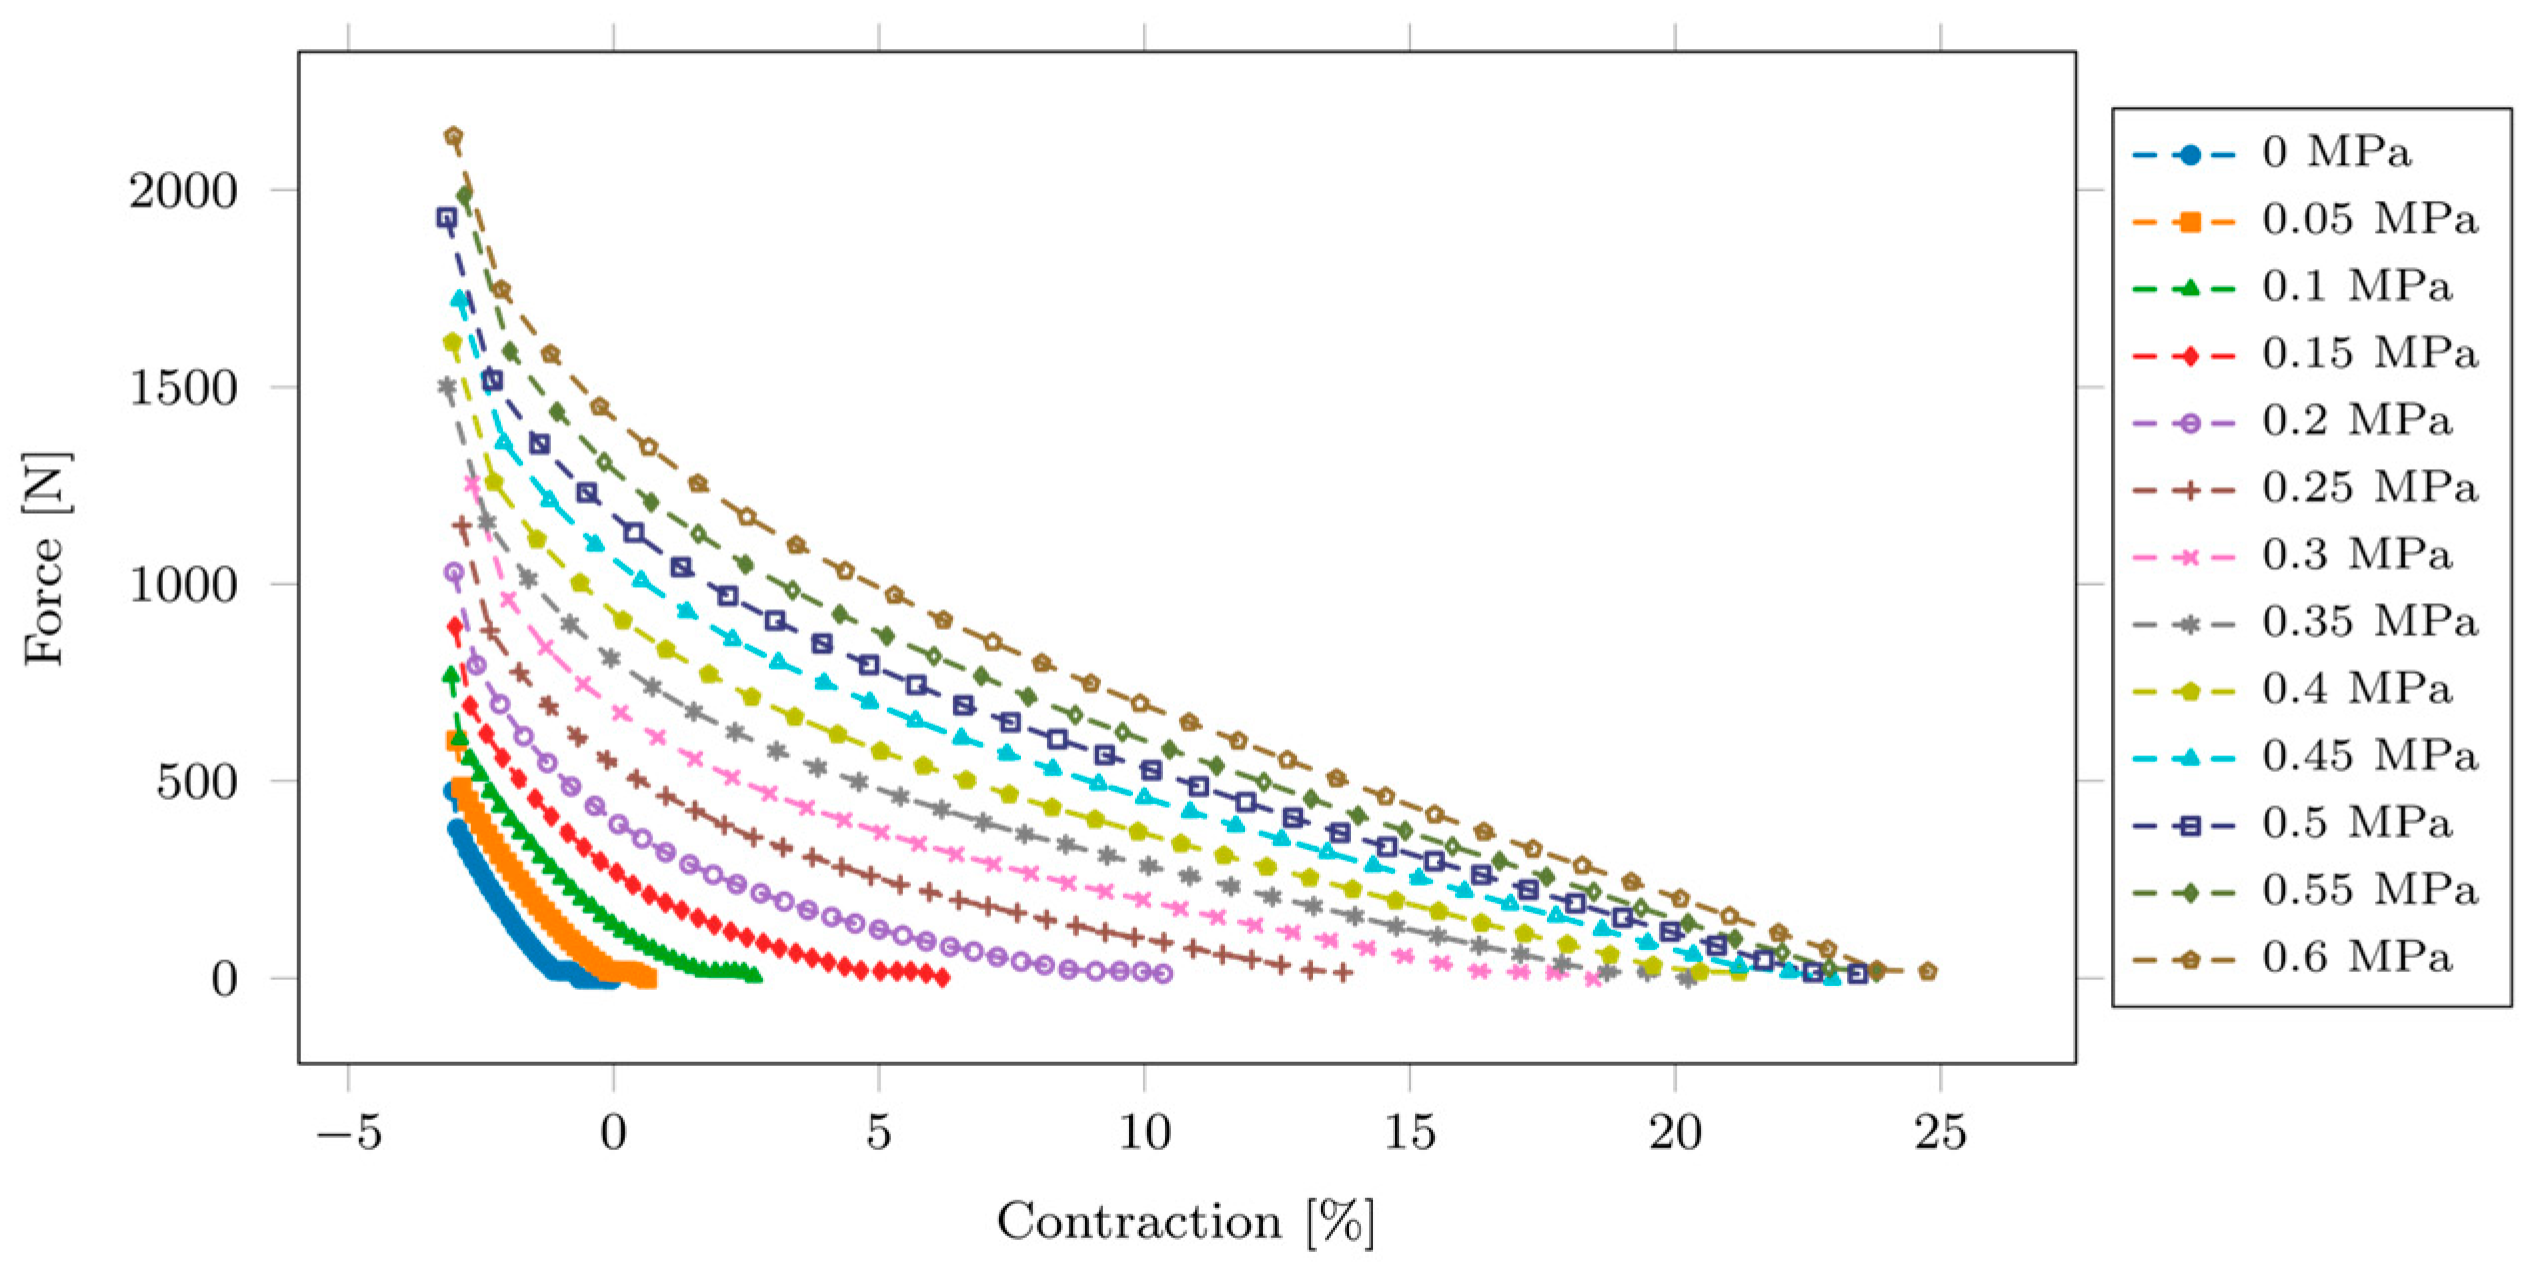
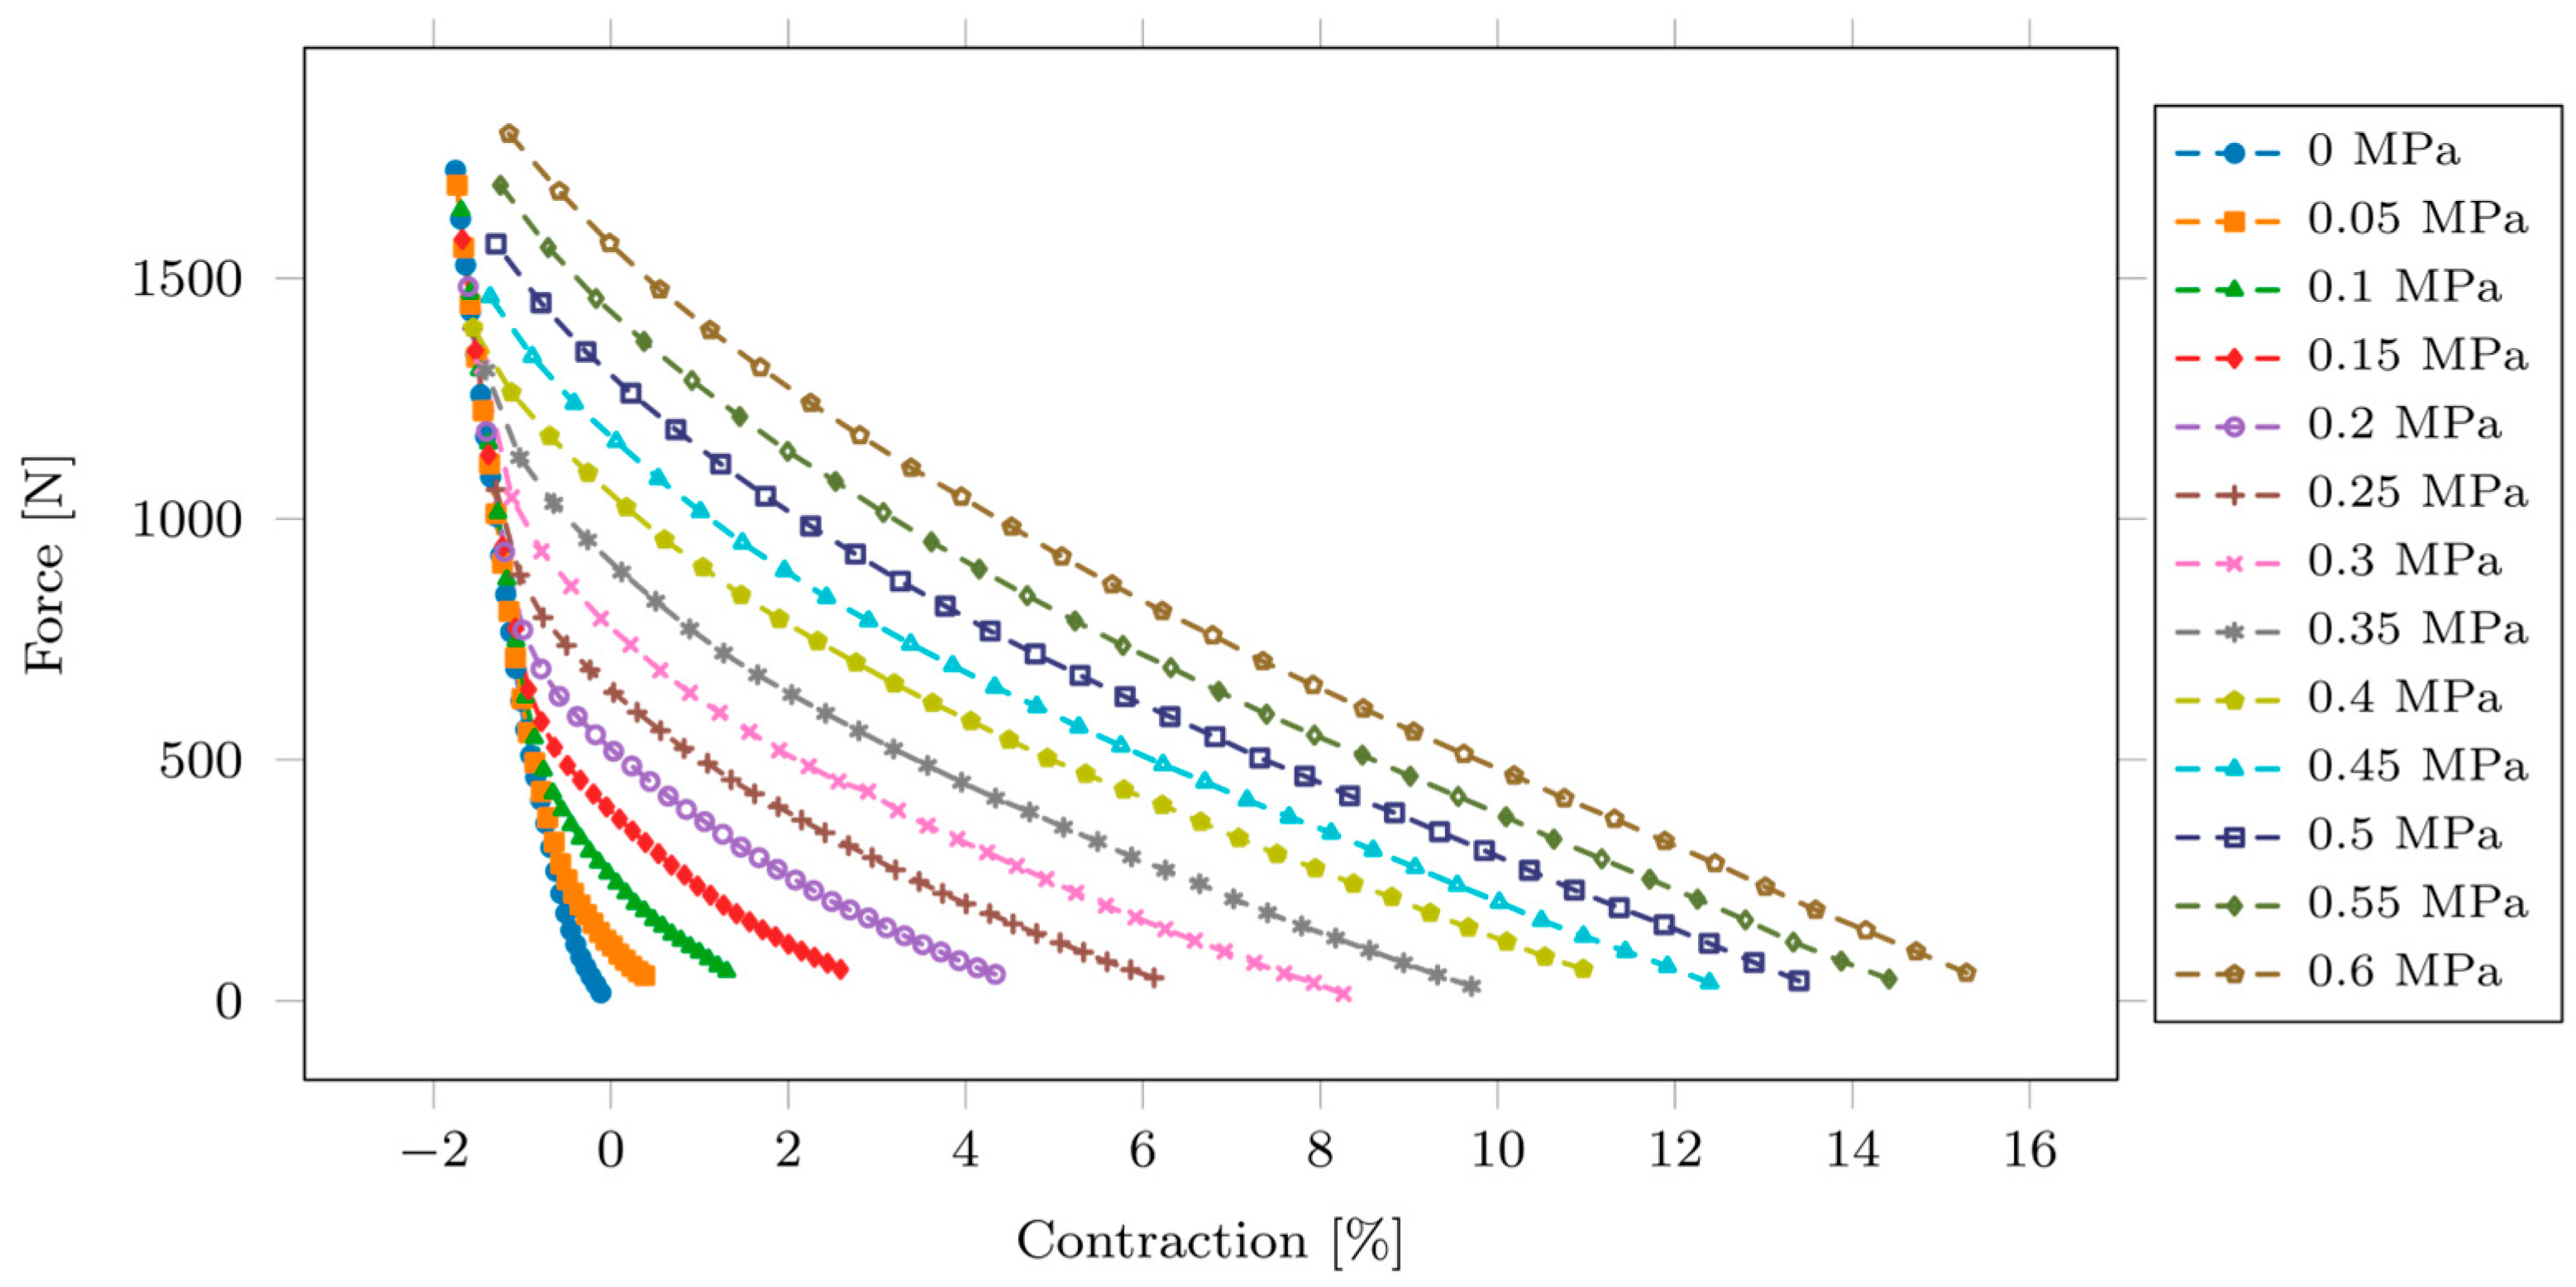
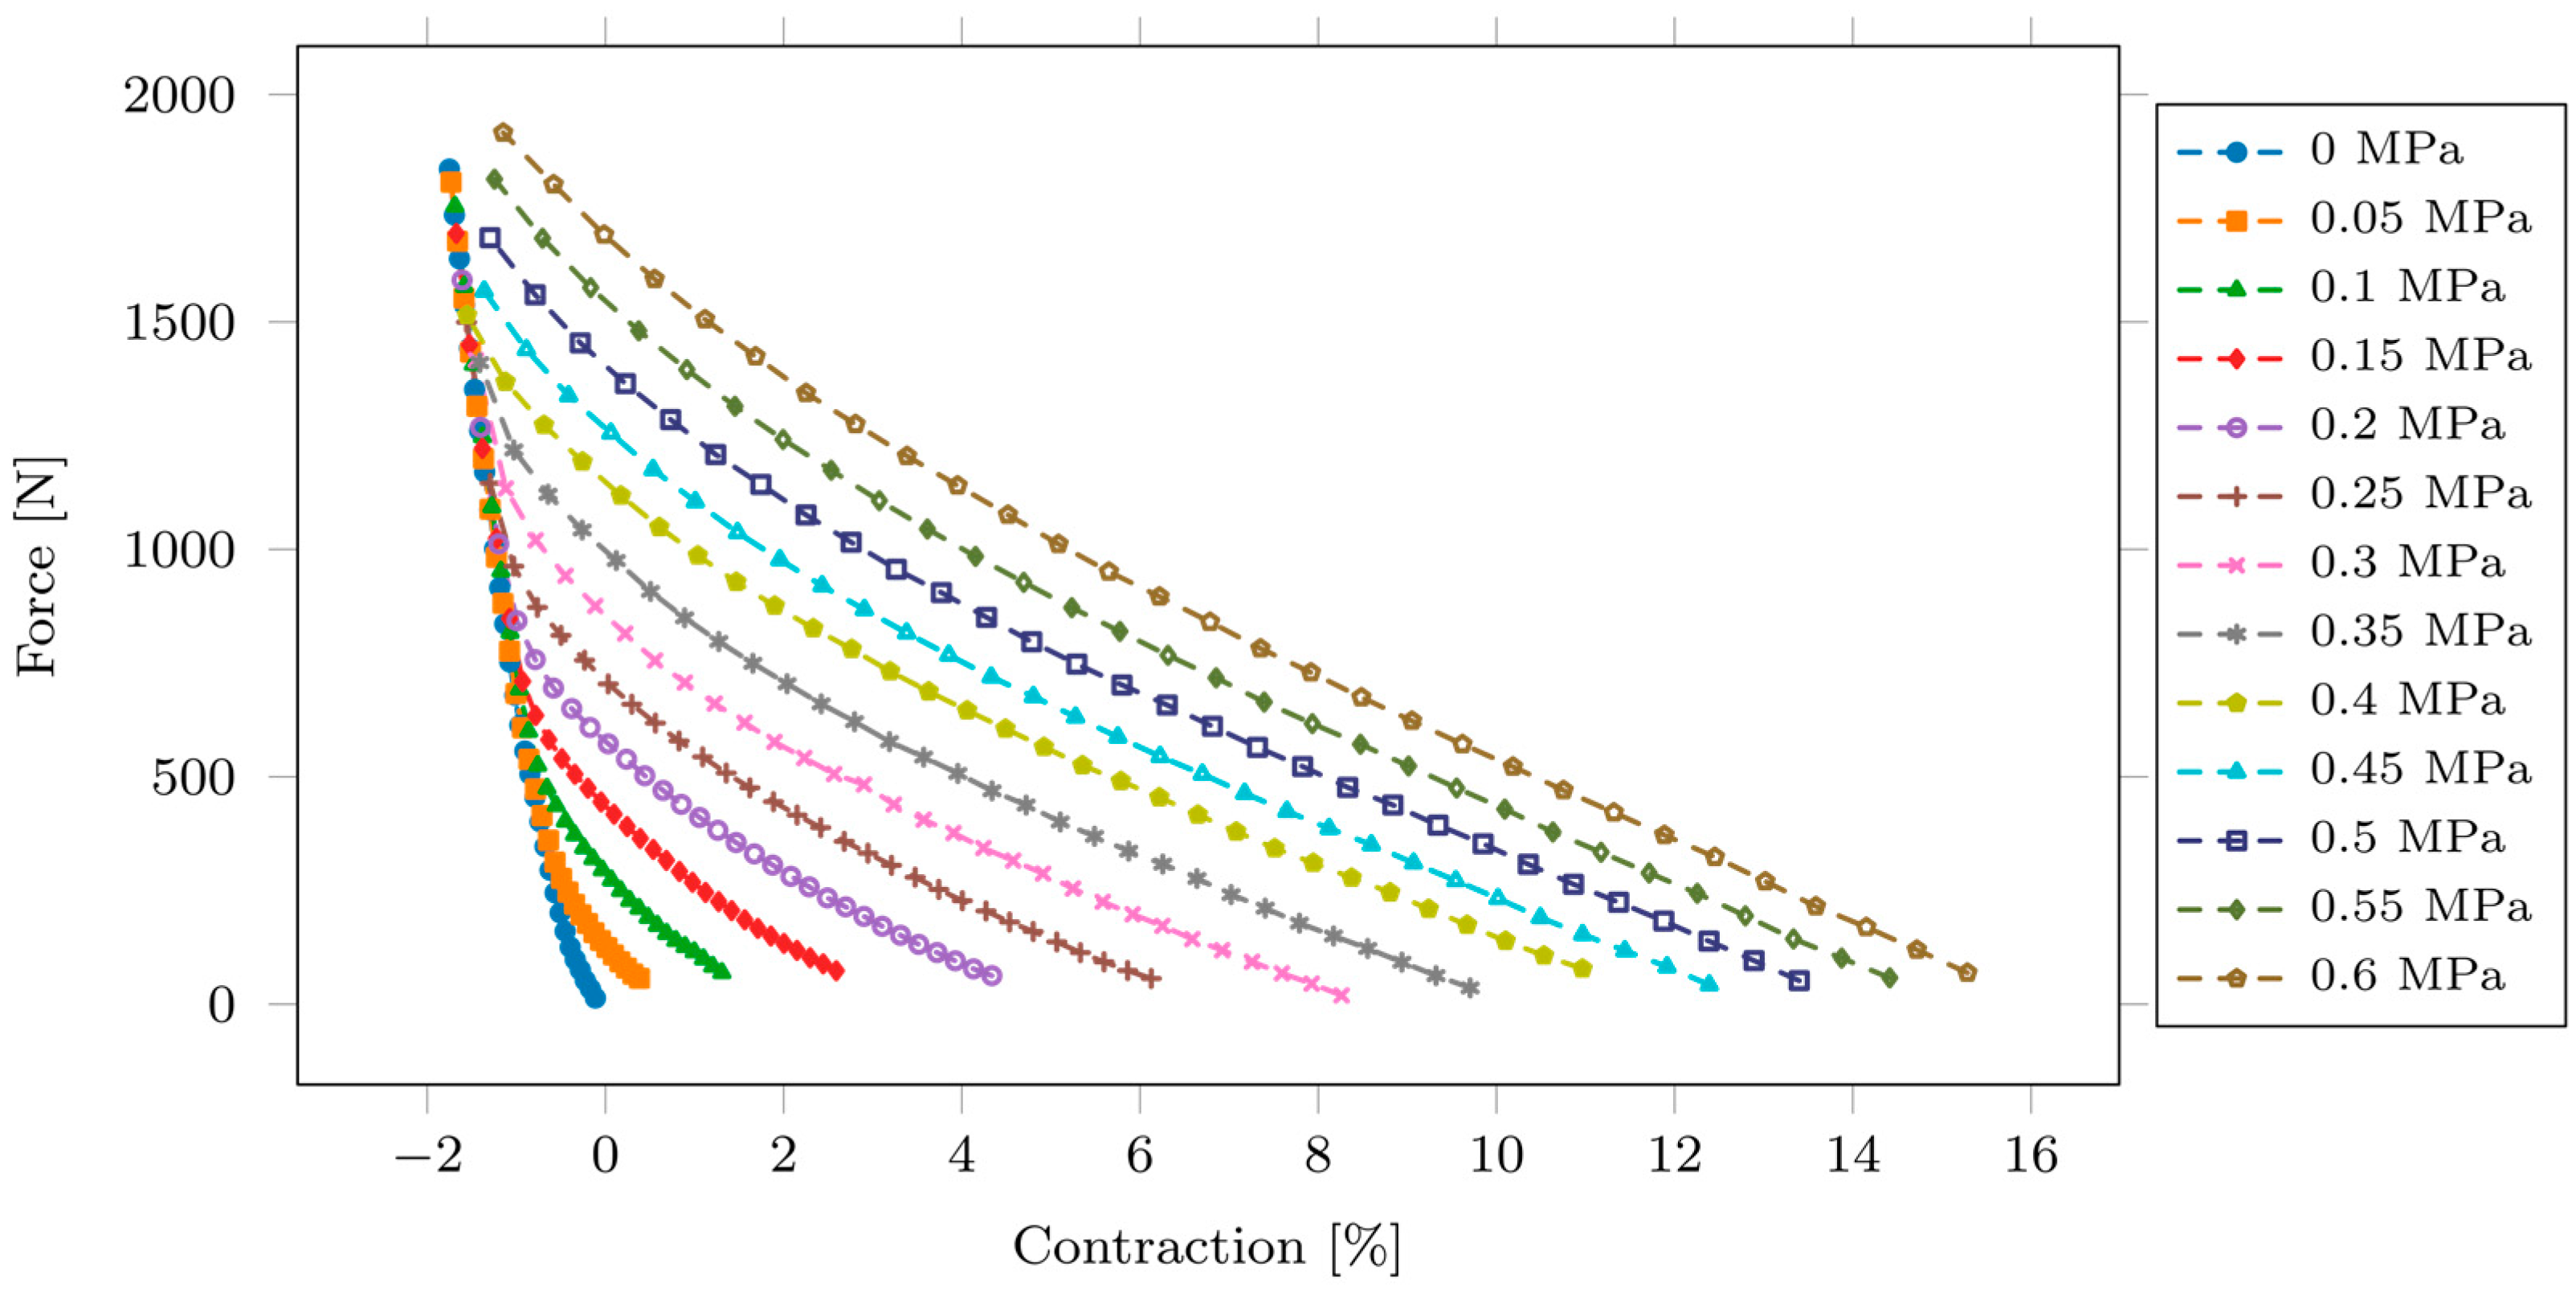
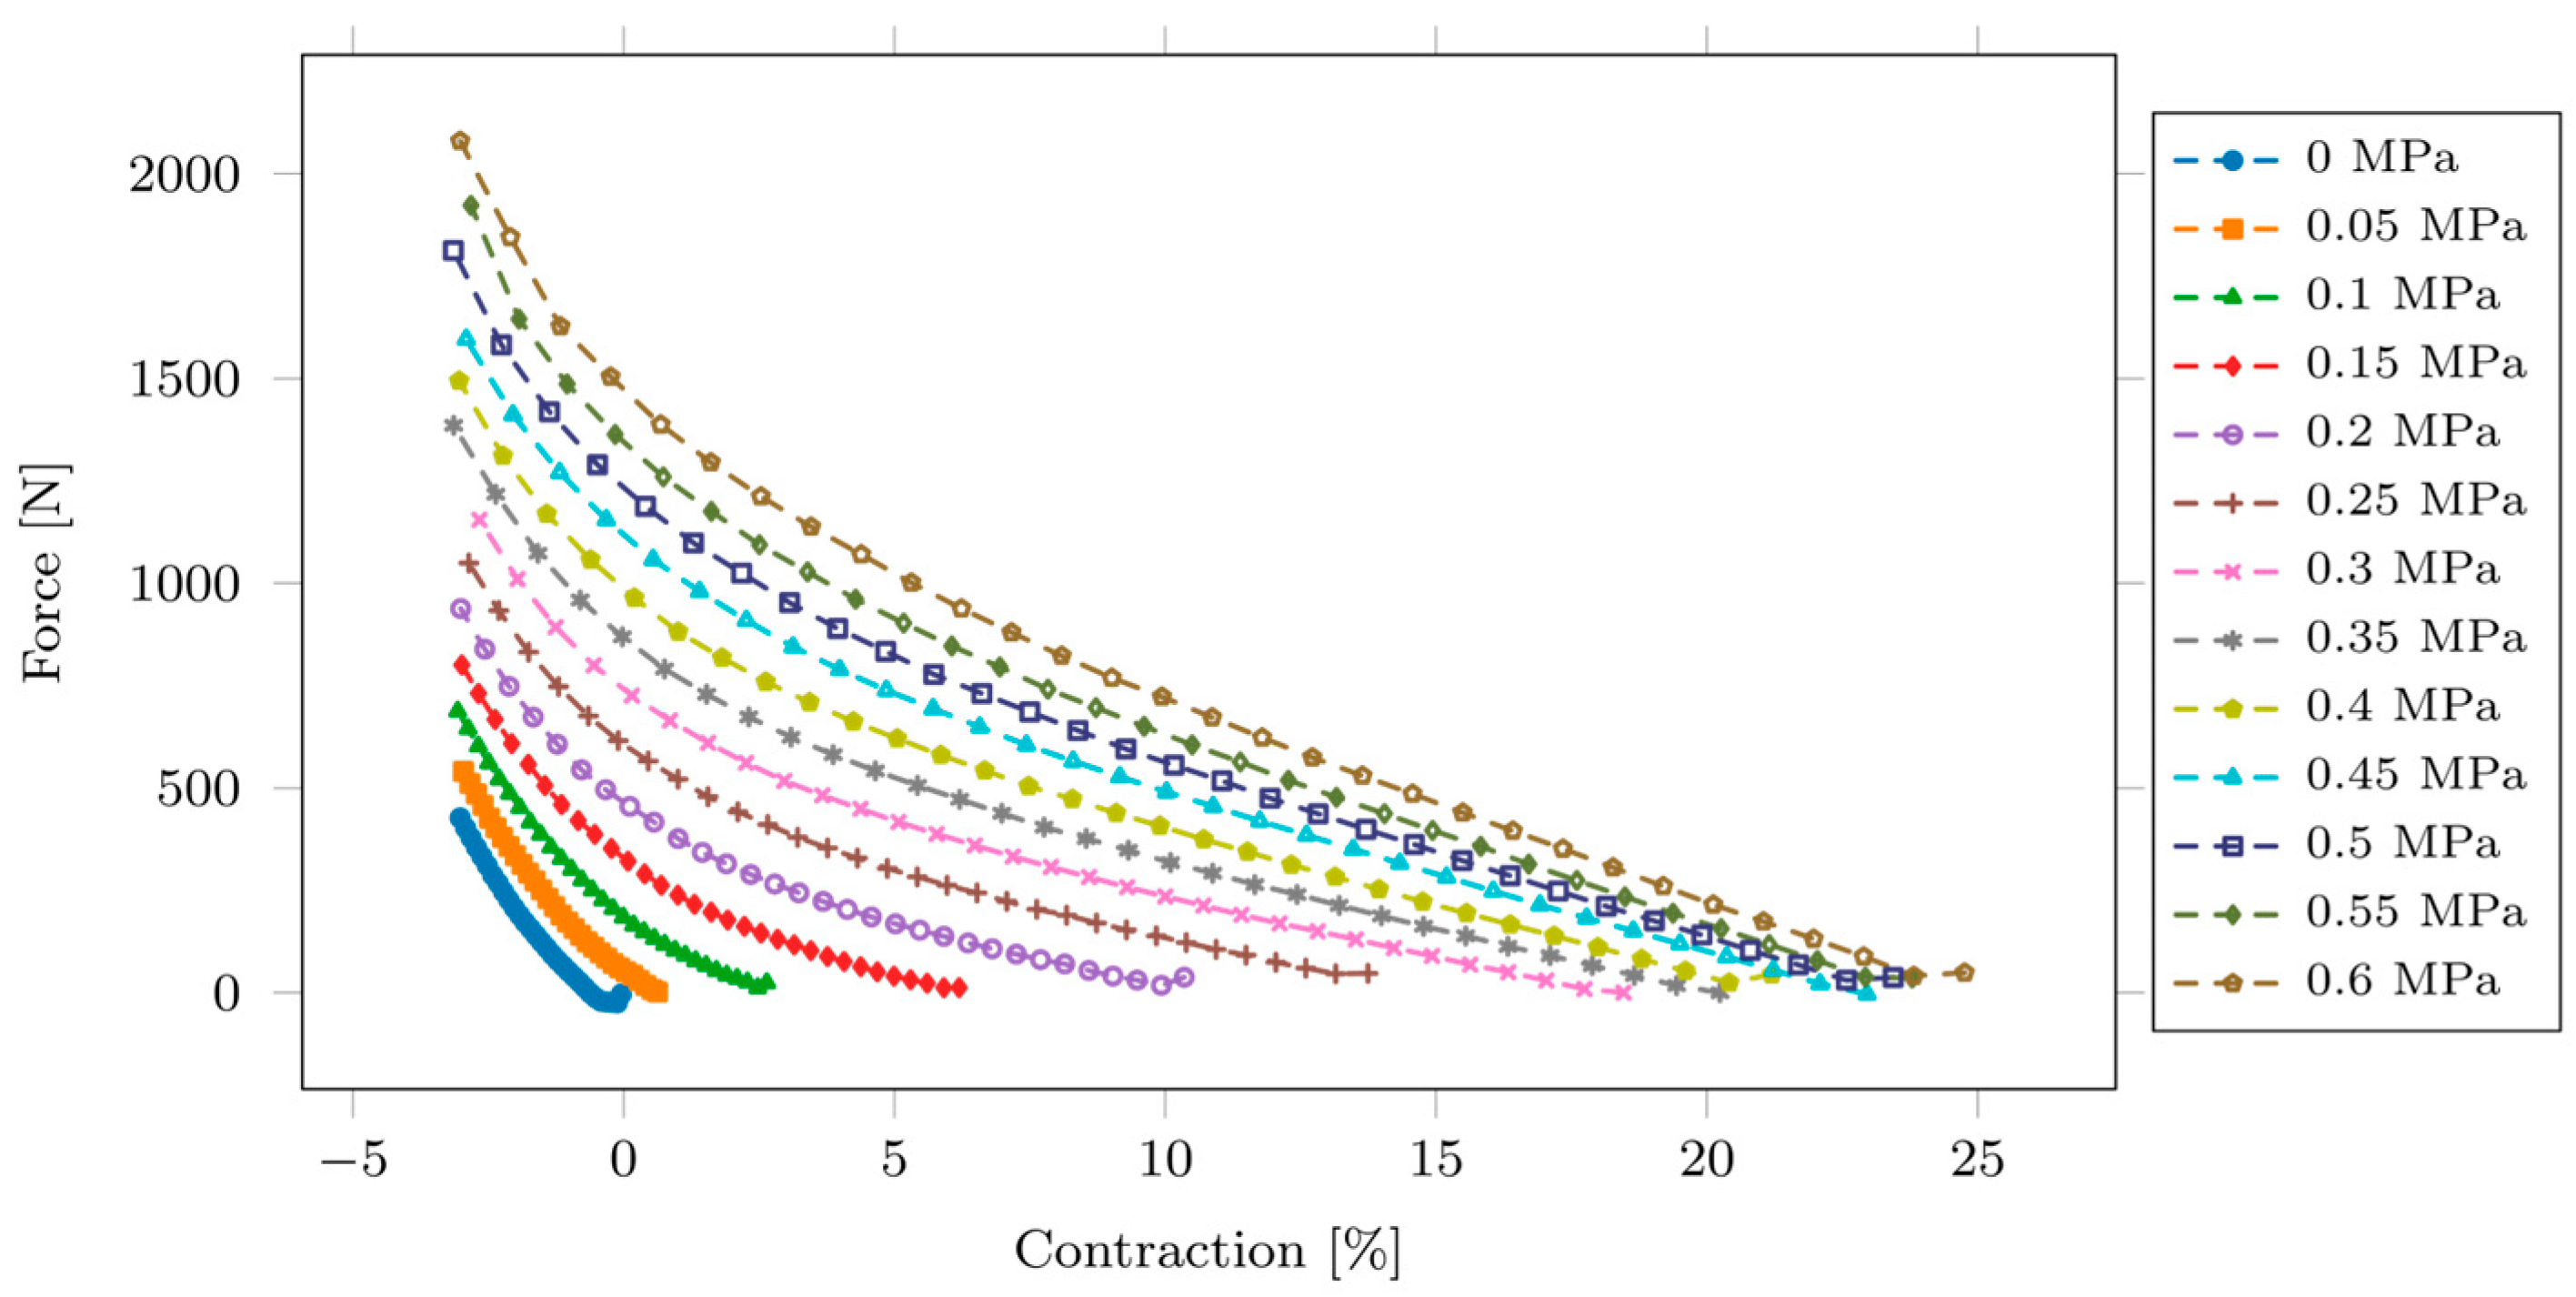
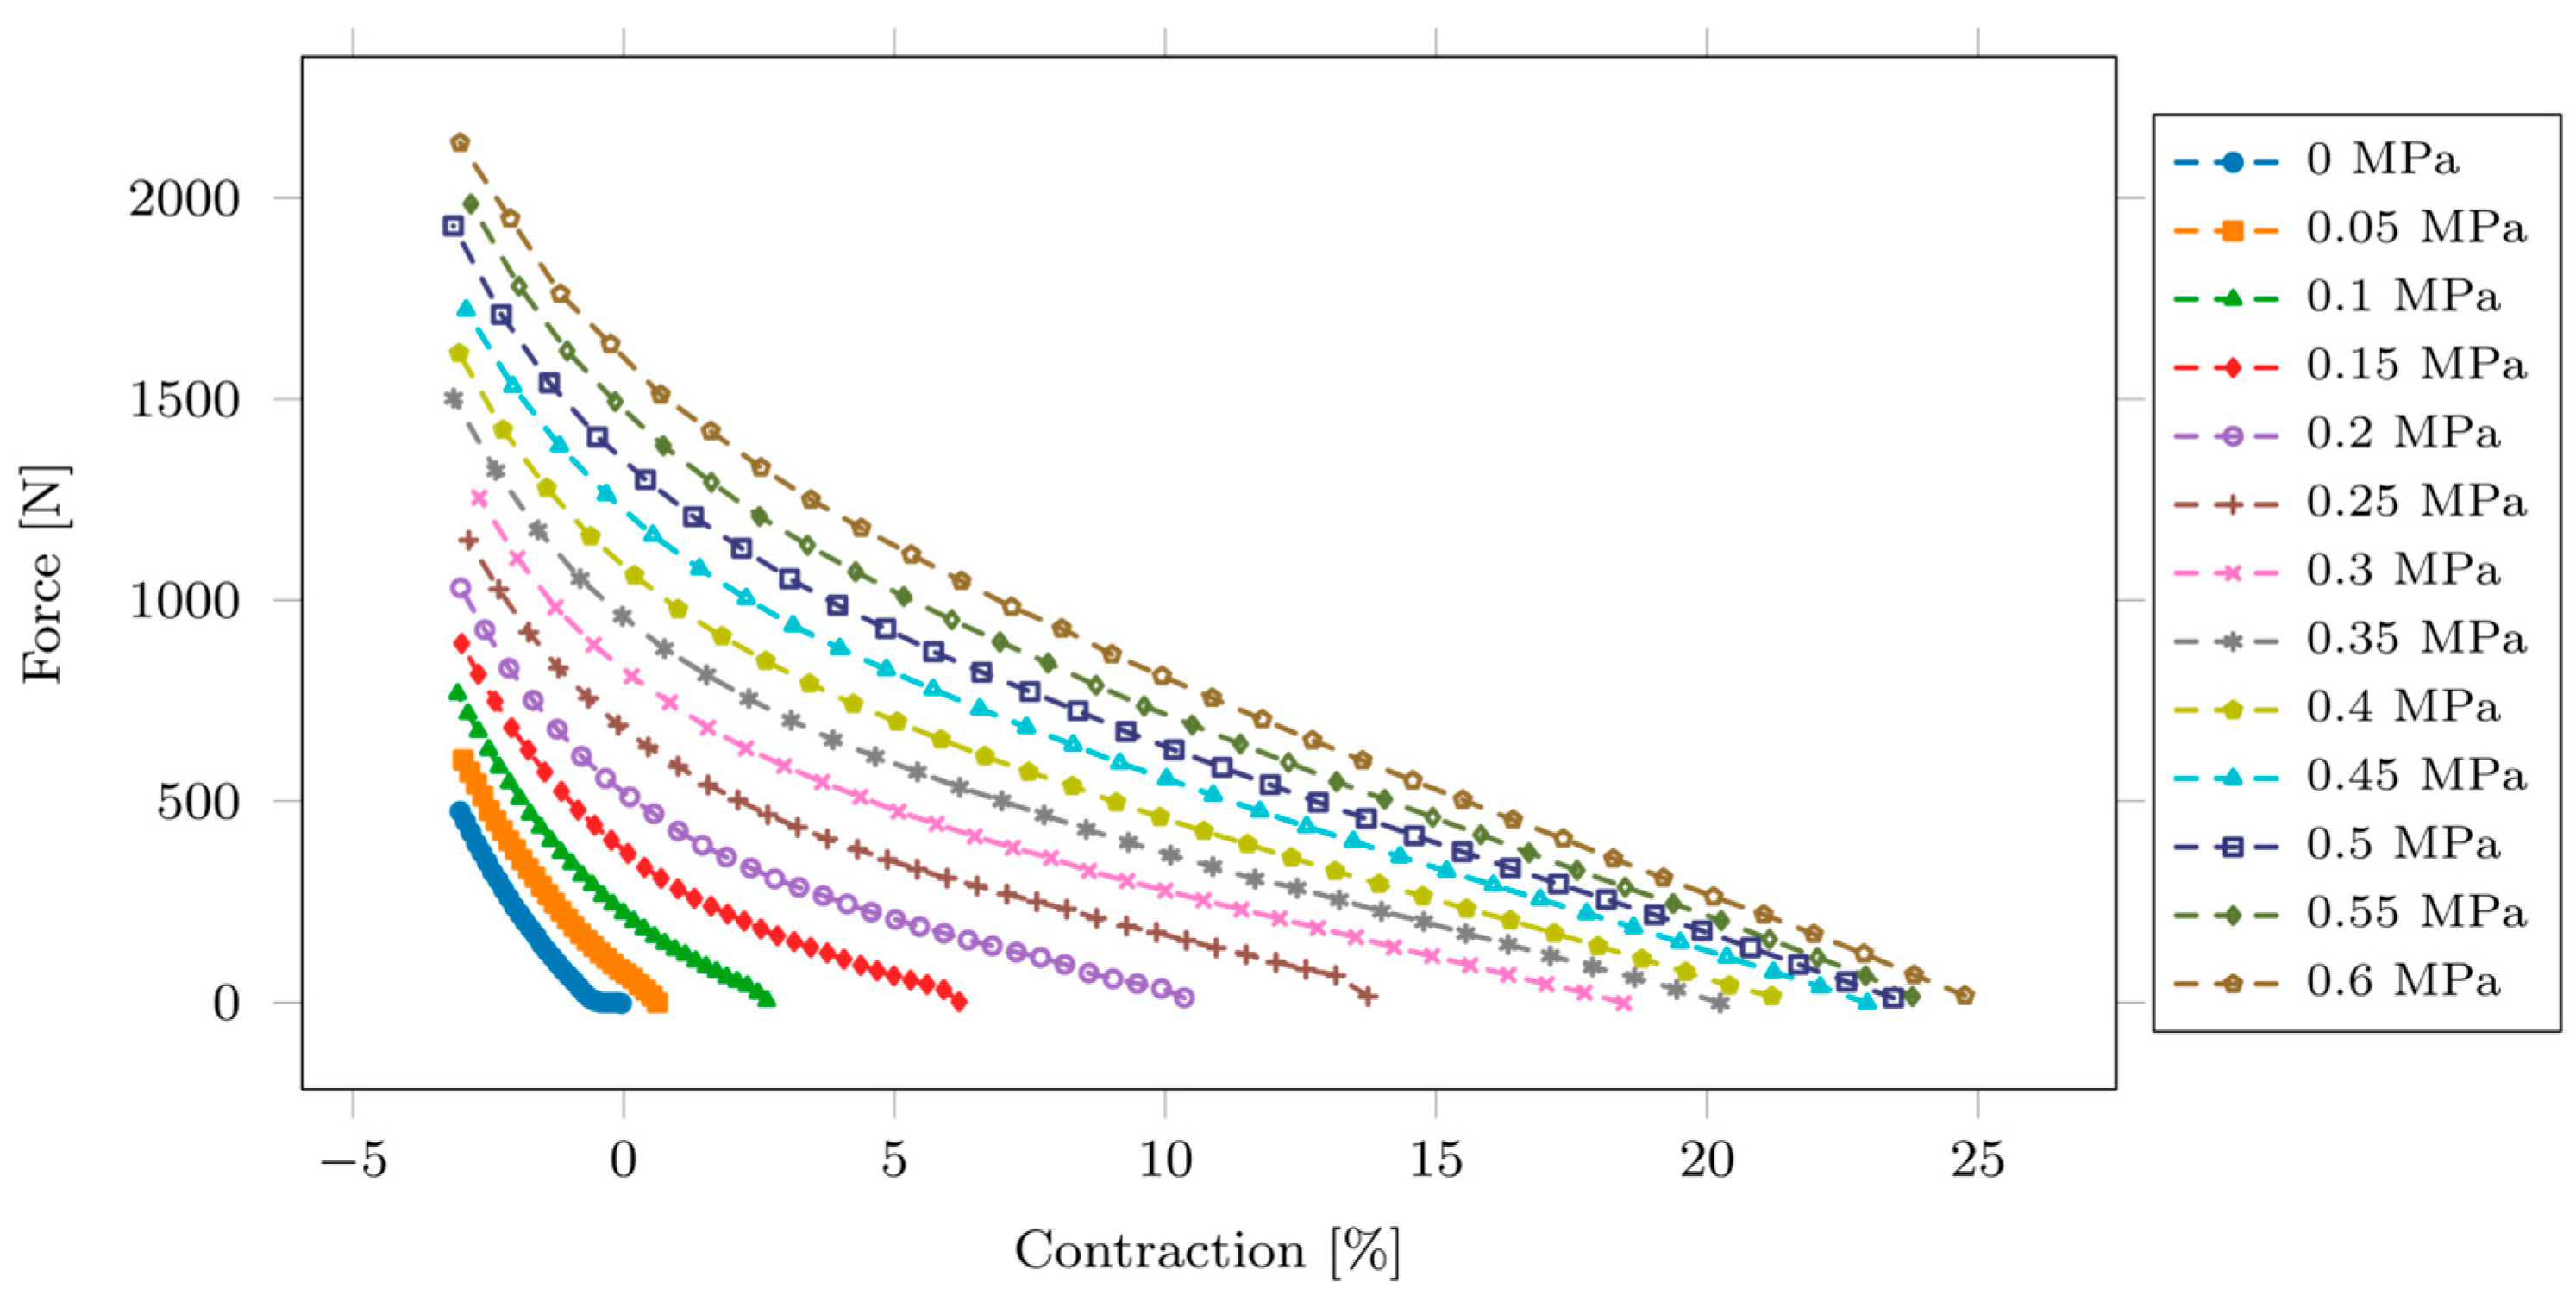
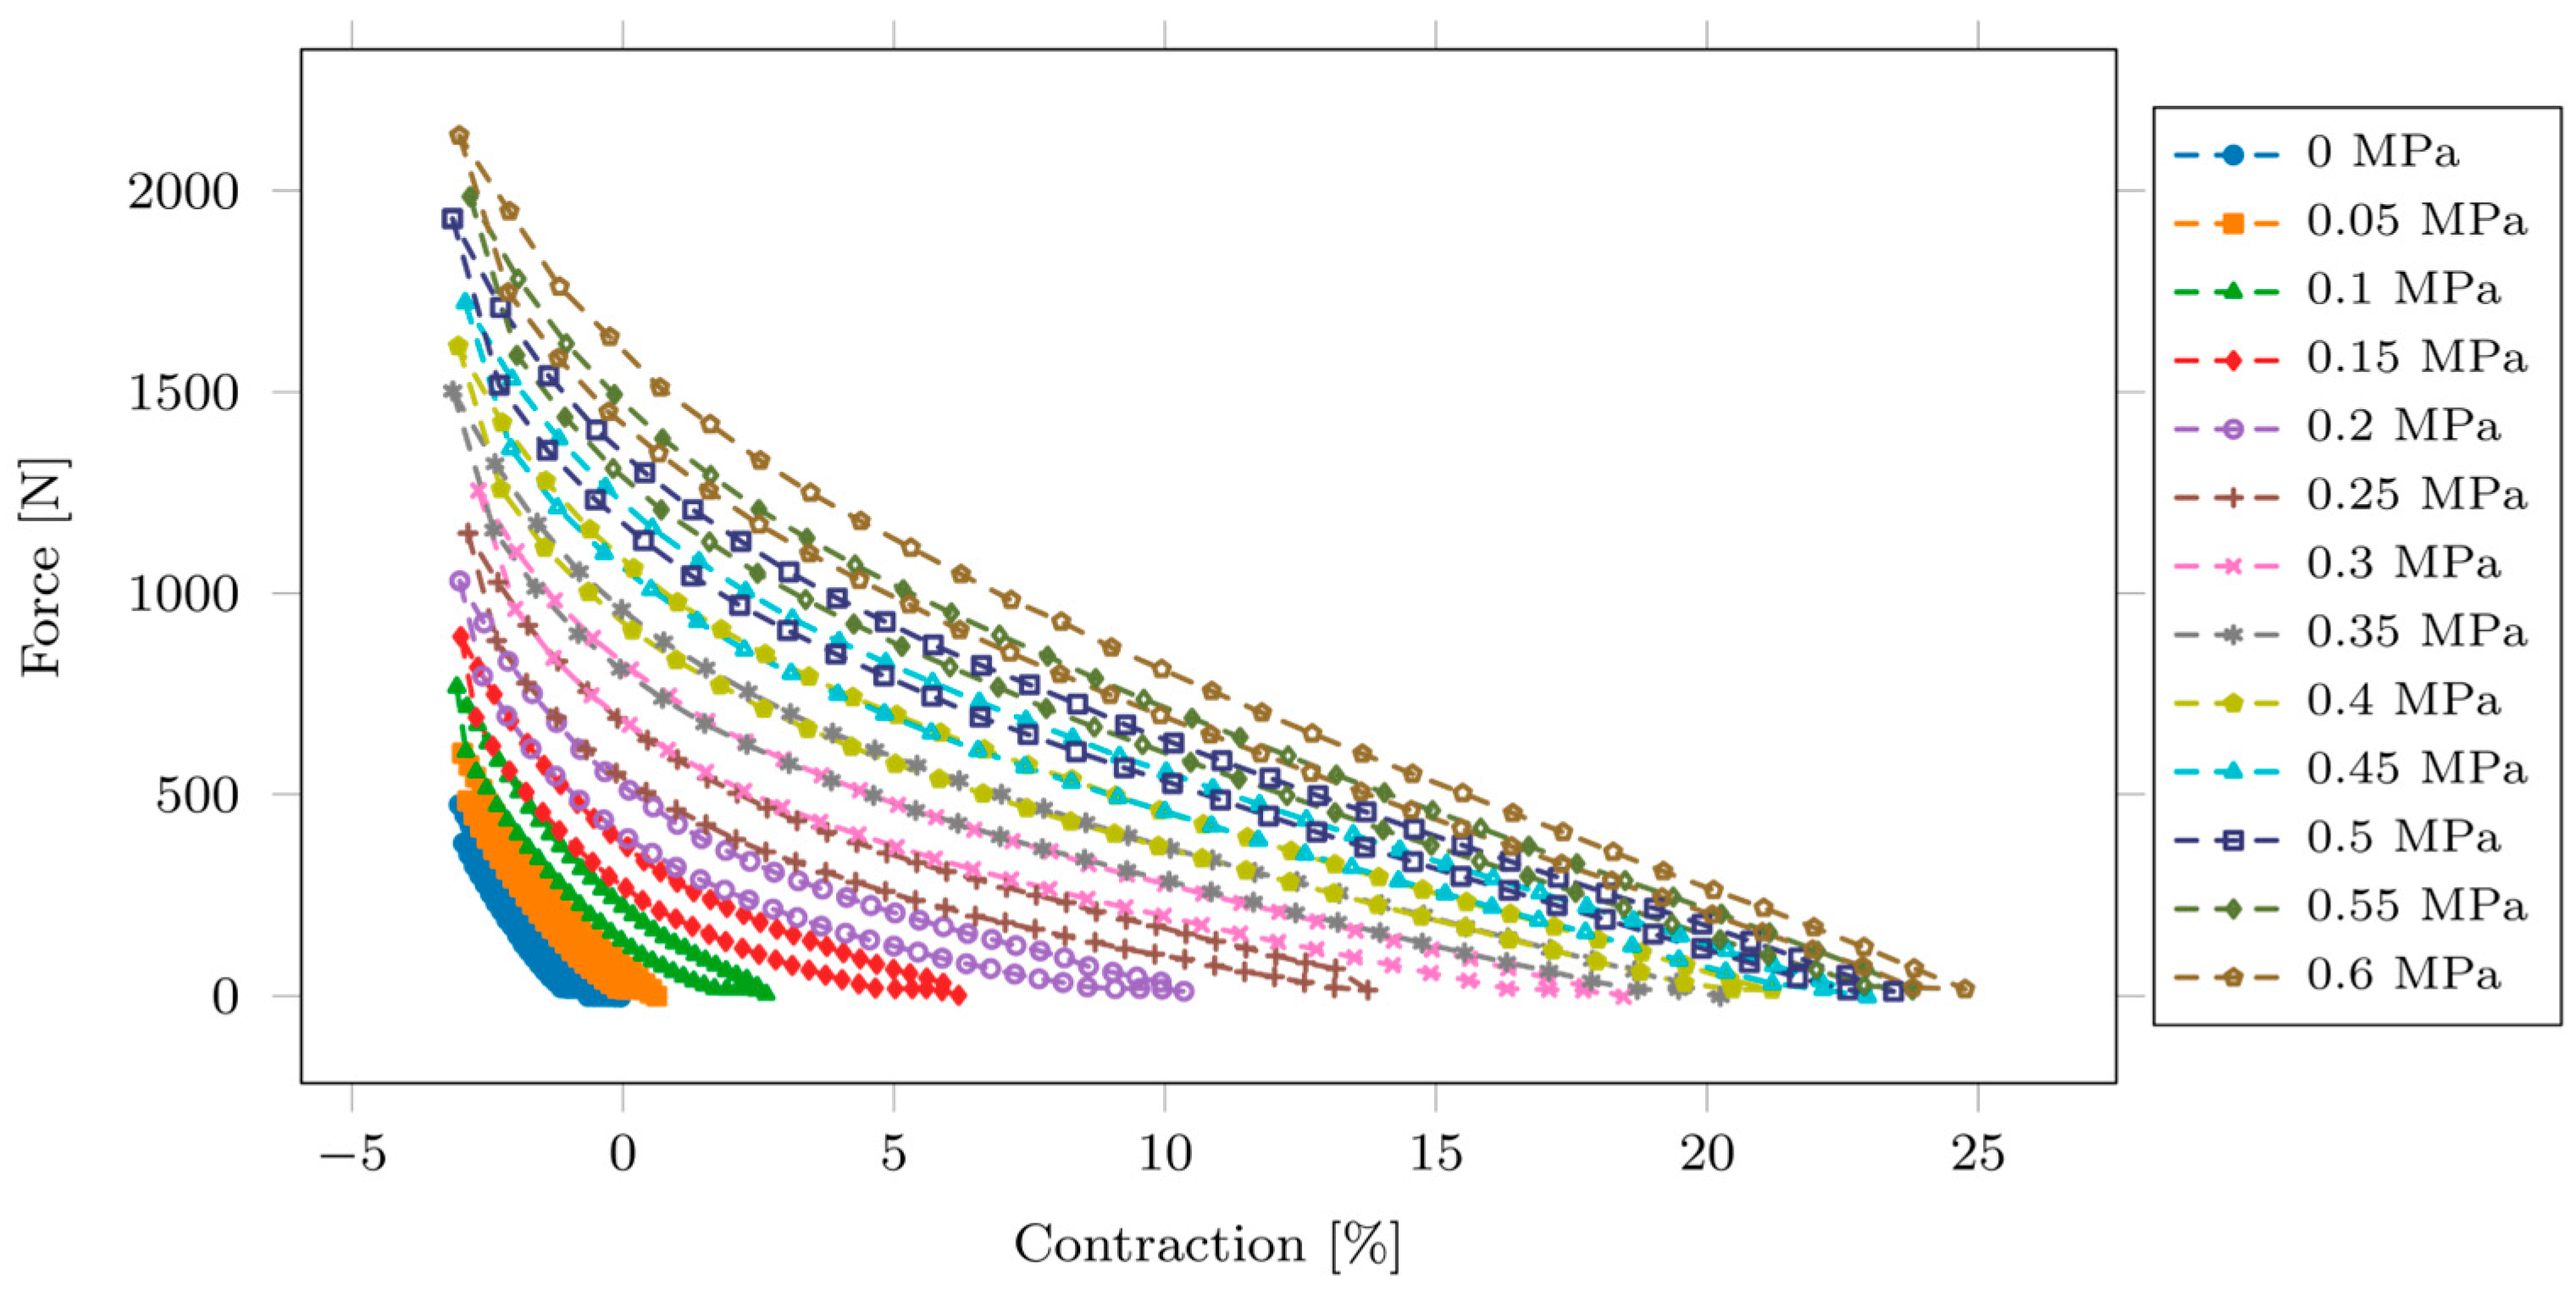
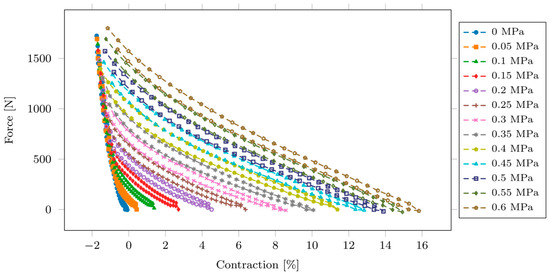
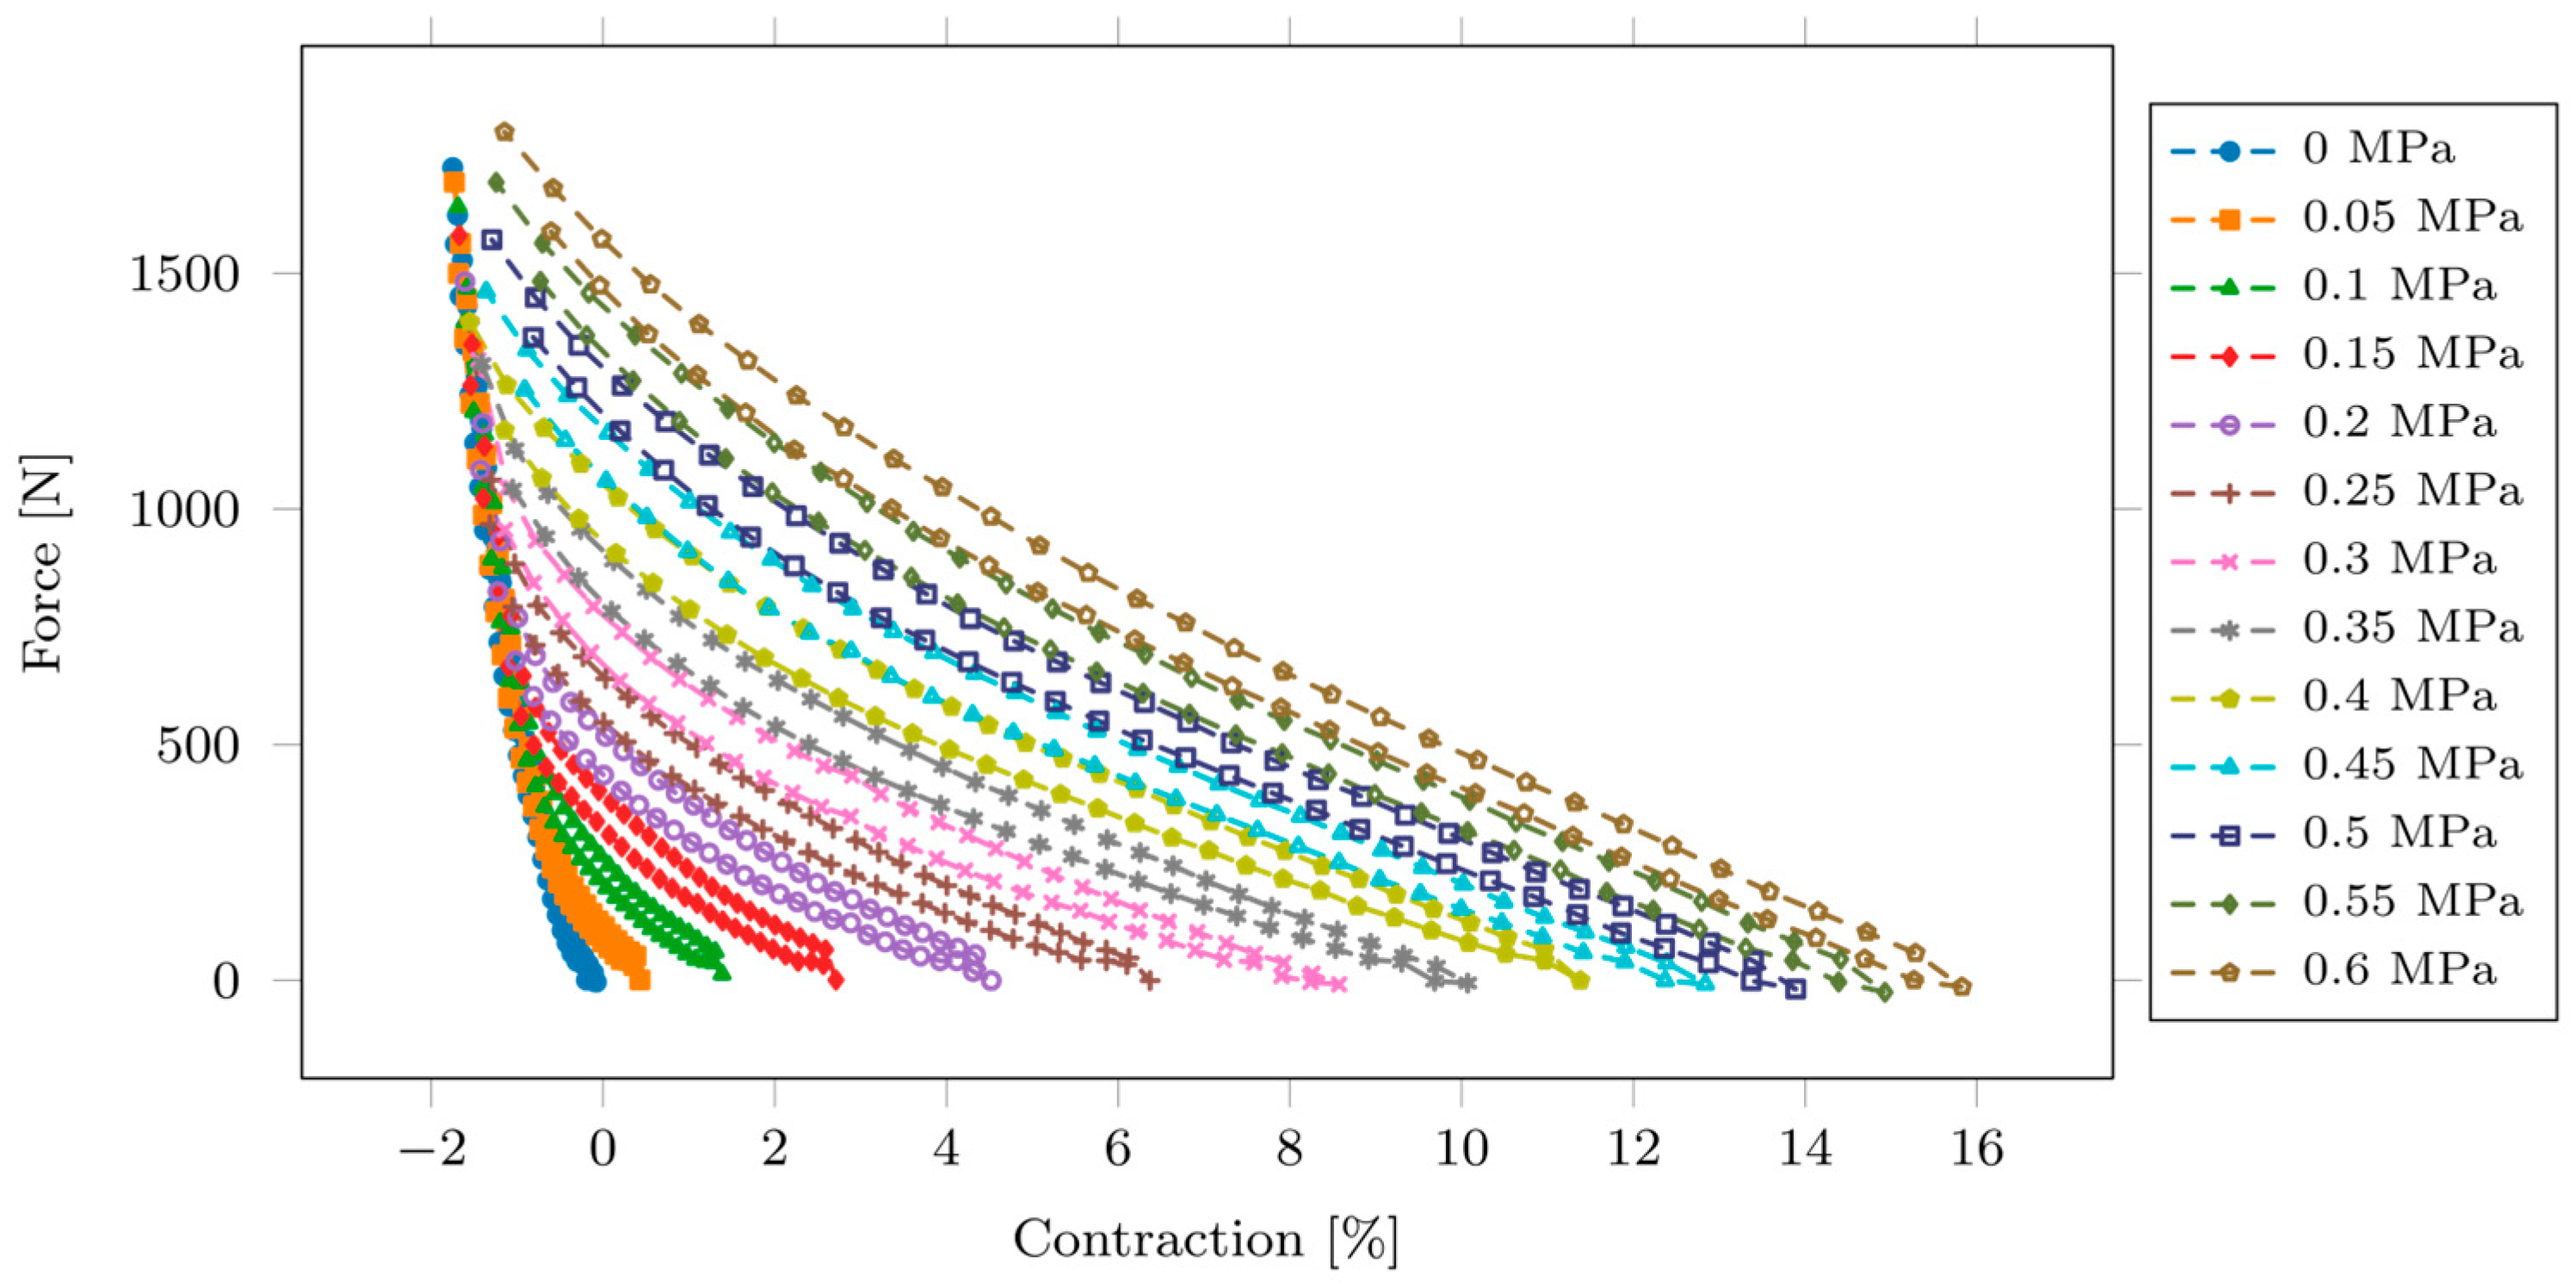
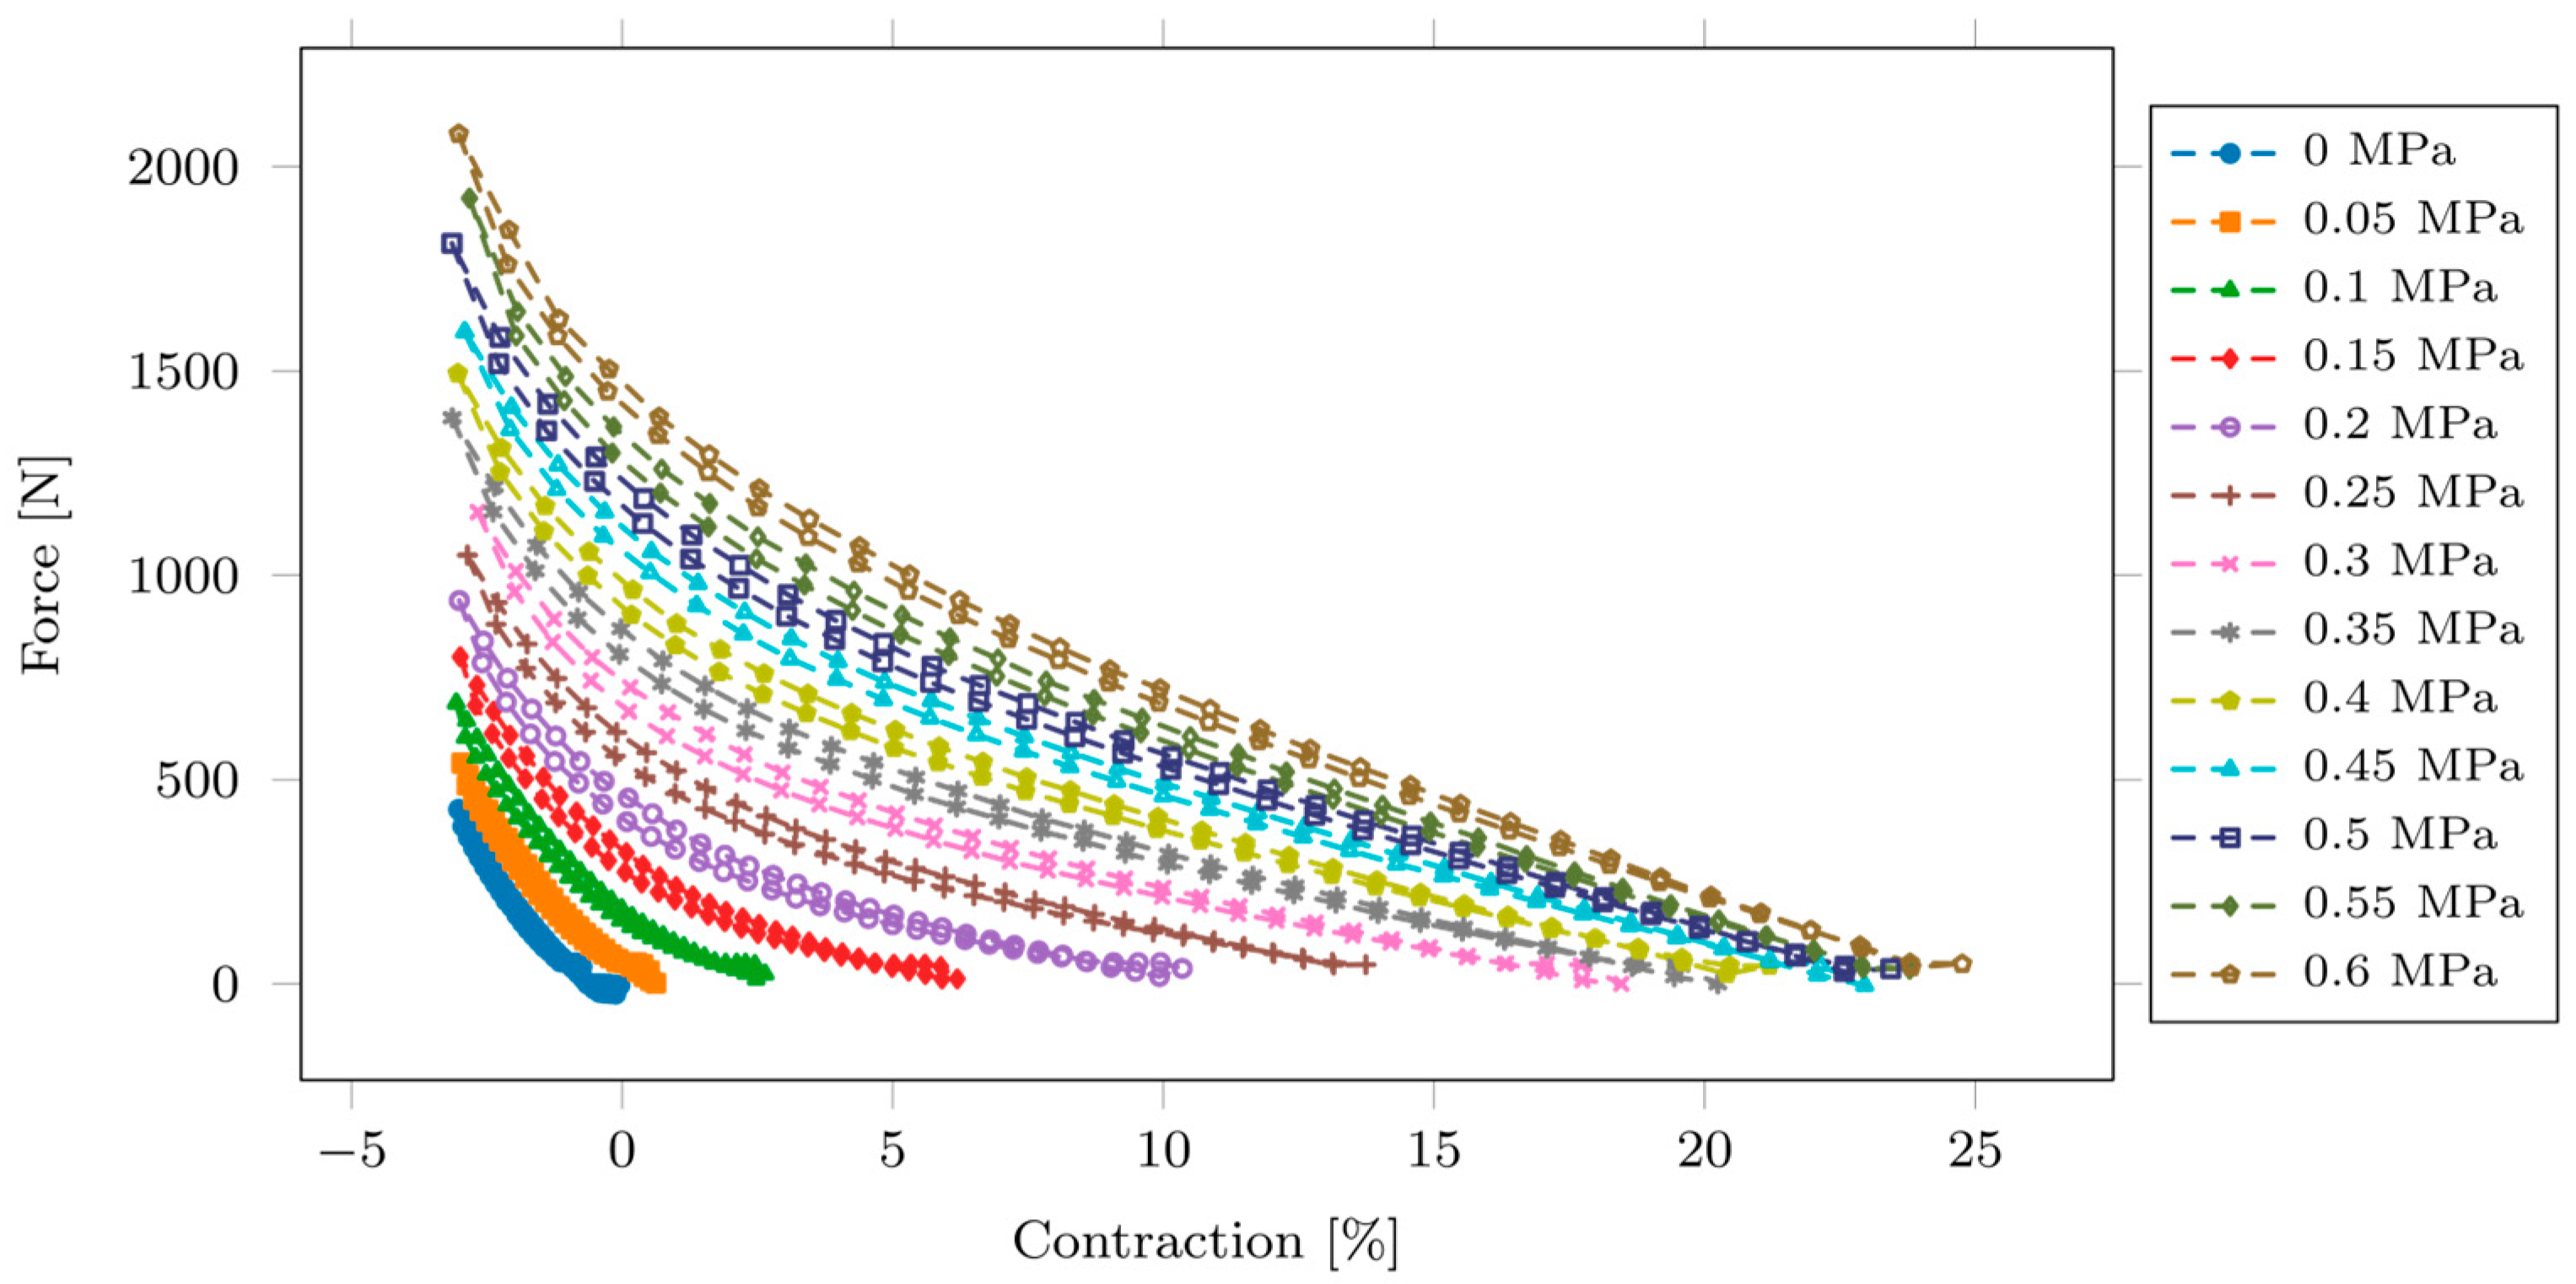
Figure 8, Figure 9, Figure 10 and Figure 11 show the force–contraction curves for the CPAM and the commercial DMSP-20-200N muscle, respectively, during the contraction (unloading) path across all 13 pressure levels. Each curve corresponds to one pressure and represents the median of five repeats.
Figure 8.
Force–contraction curves of the CPAM actuator during contraction (load cell force).
Figure 9.
Force–contraction curves of the CPAM actuator during contraction (excitation force).
Figure 10.
Force–contraction curves of the DMSP actuator during contraction (load cell force).
Figure 11.
Force–contraction curves of the DMSP actuator during contraction (excitation force).
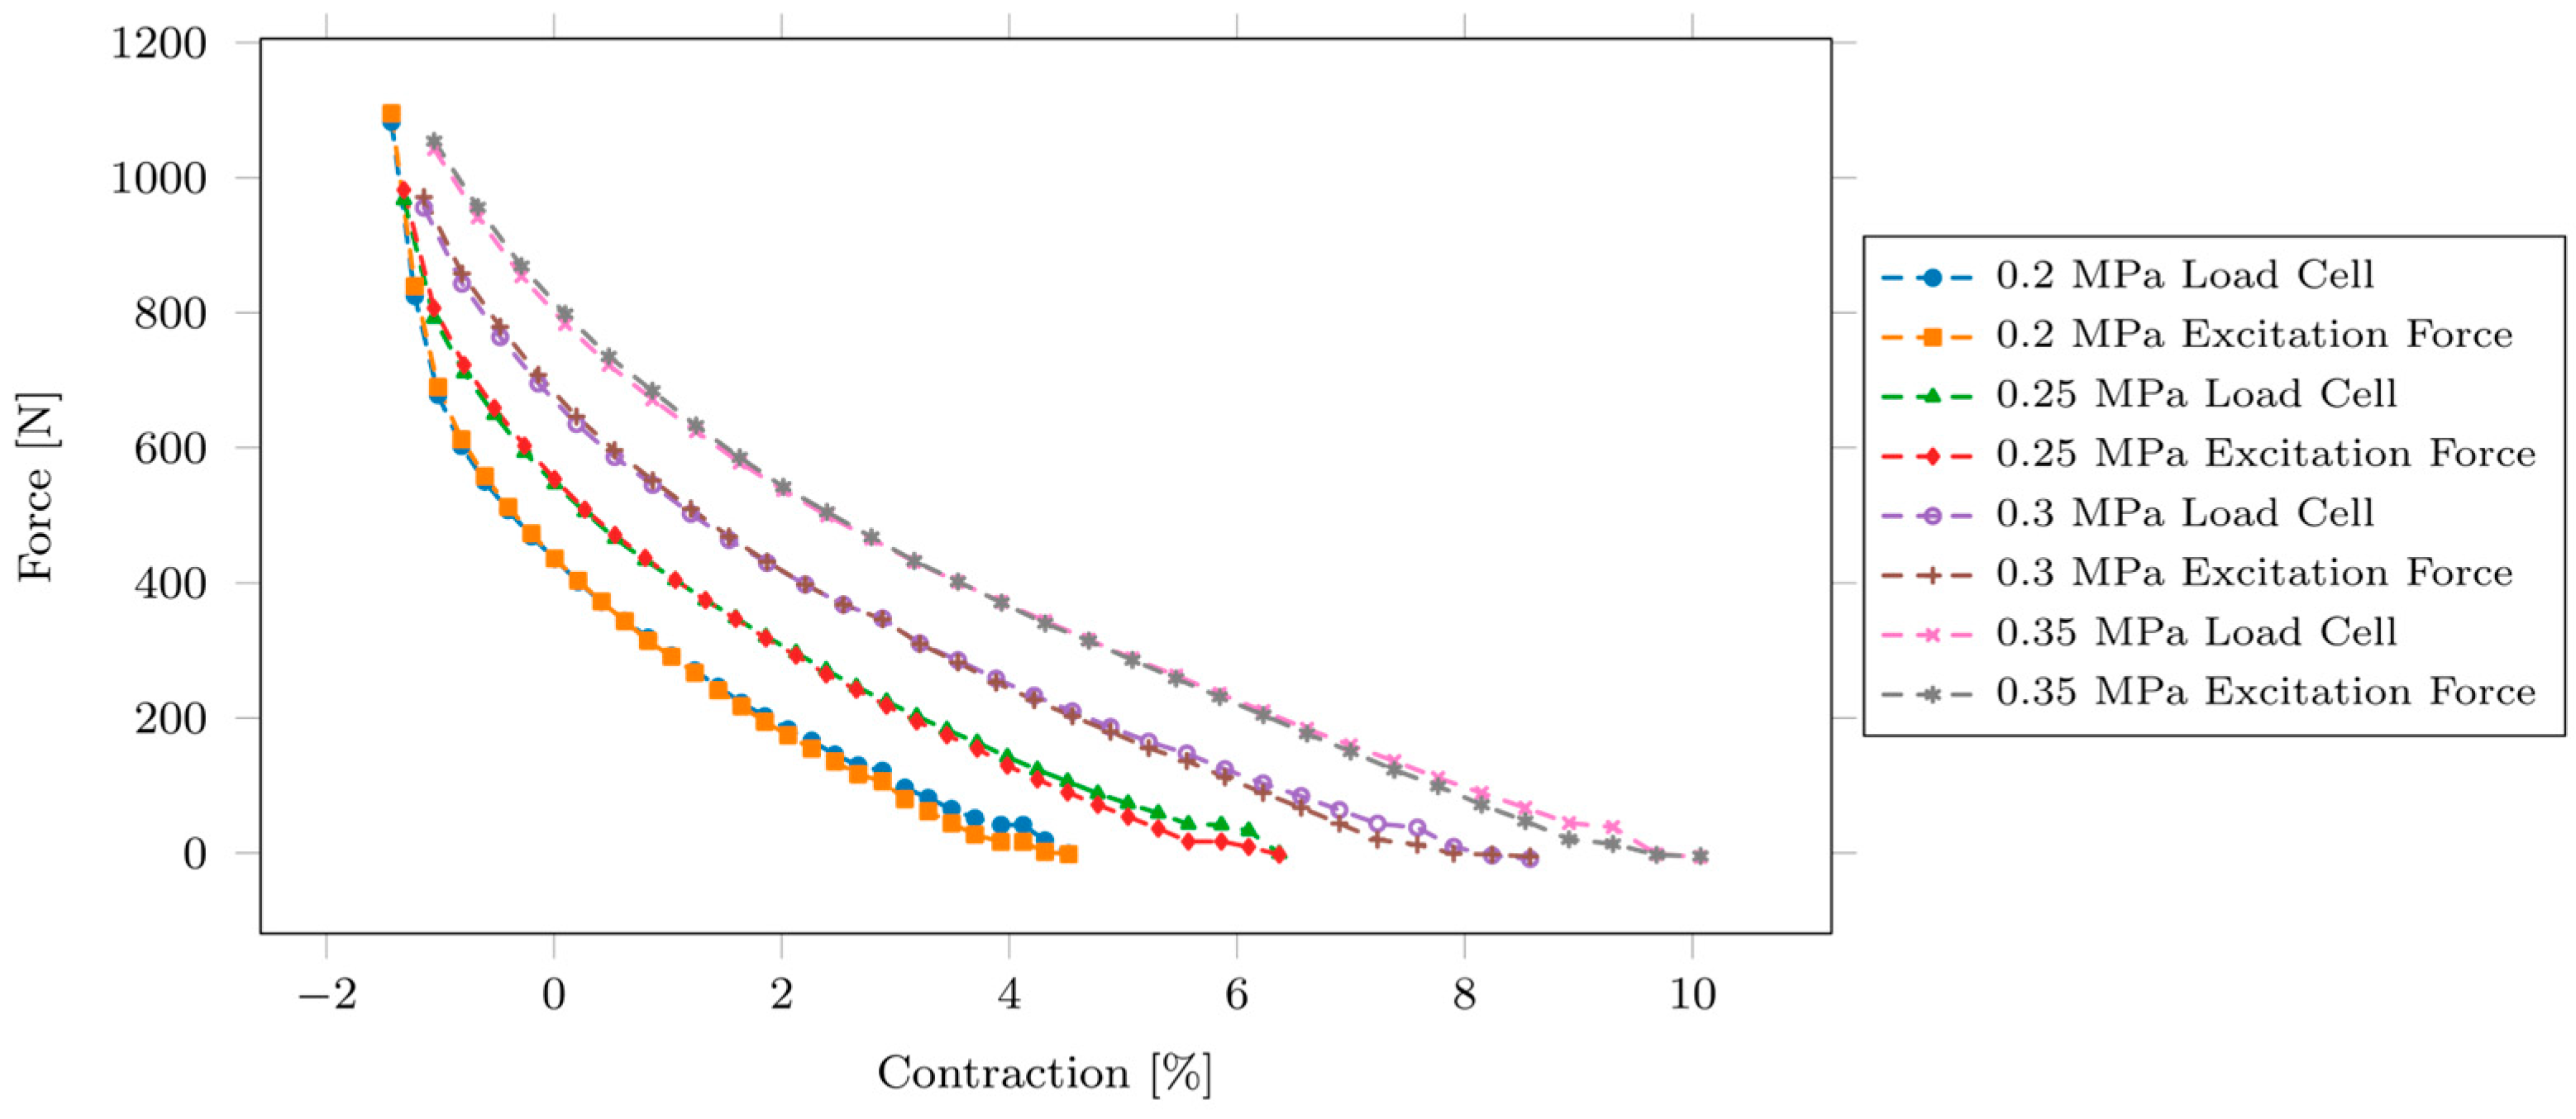
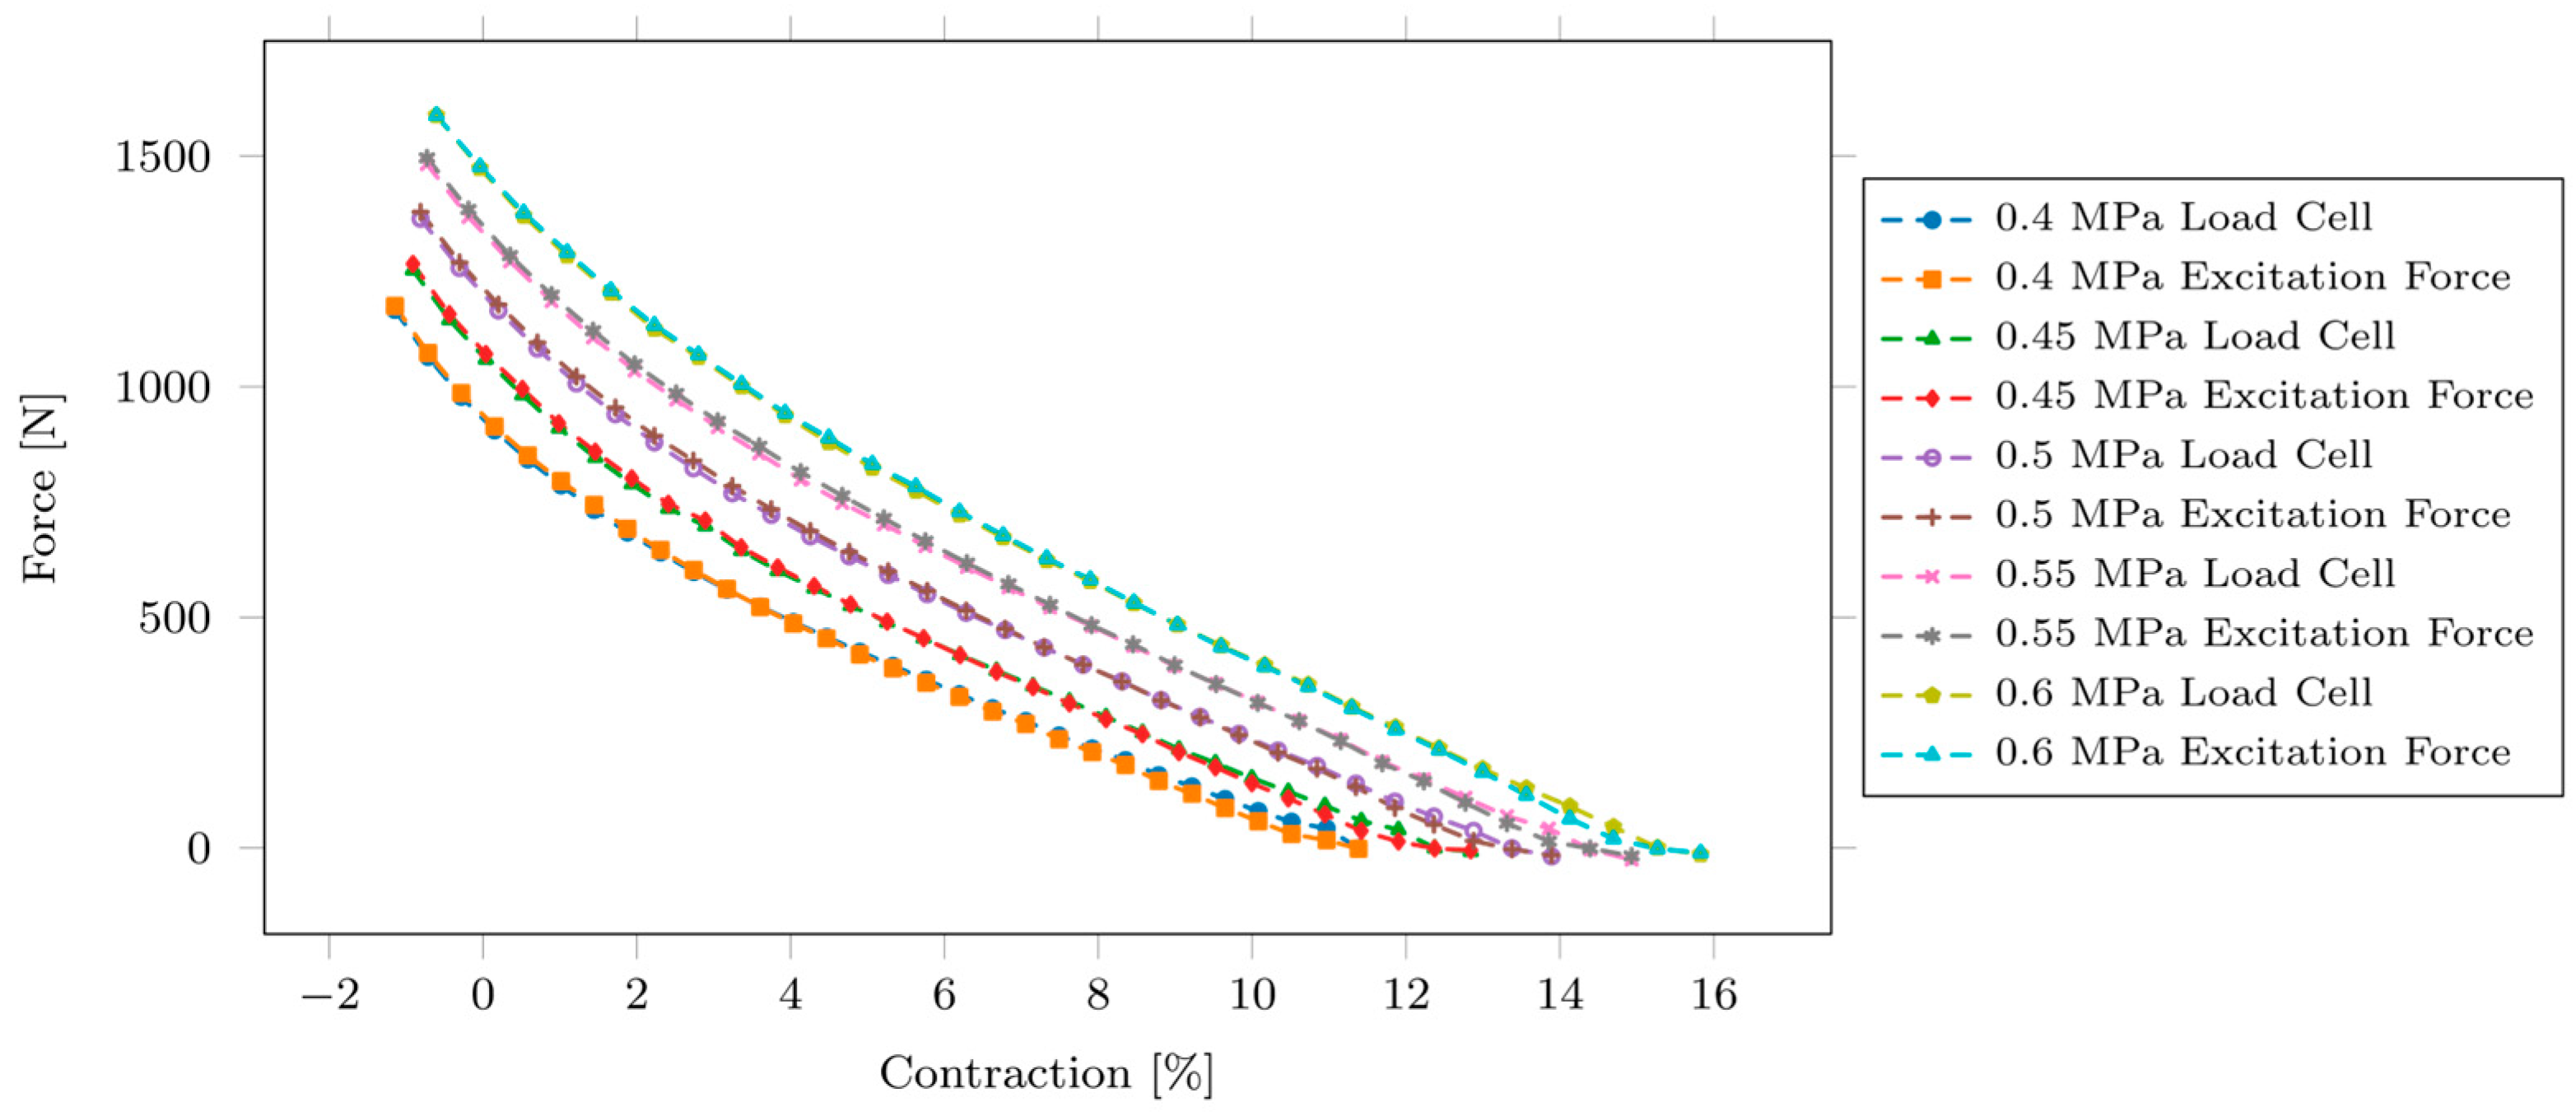
Across the tested pressure range, both actuators exhibit the expected monotonic decrease in force with contraction at fixed pressure and an approximately linear increase in force with pressure at fixed contraction. Two consistent differences can be observed:
- For a given pressure, the CPAM contracts almost 10% less than the commercial muscle, reflecting its higher overall stiffness due to the internal spring and rod.
- For a given contraction and pressure, the CPAM produces a higher force than the commercial muscle at low pressures, indicating that part of the load is carried by the internal spring while the outer muscle still contributes significantly.
The variability across repeats is small for both actuators, and no systematic drift over the five cycles is visible, which supports the use of median curves in the hysteresis analysis.
3.3. Loading (Expansion) Behavior
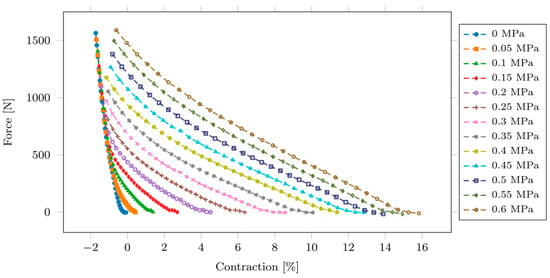
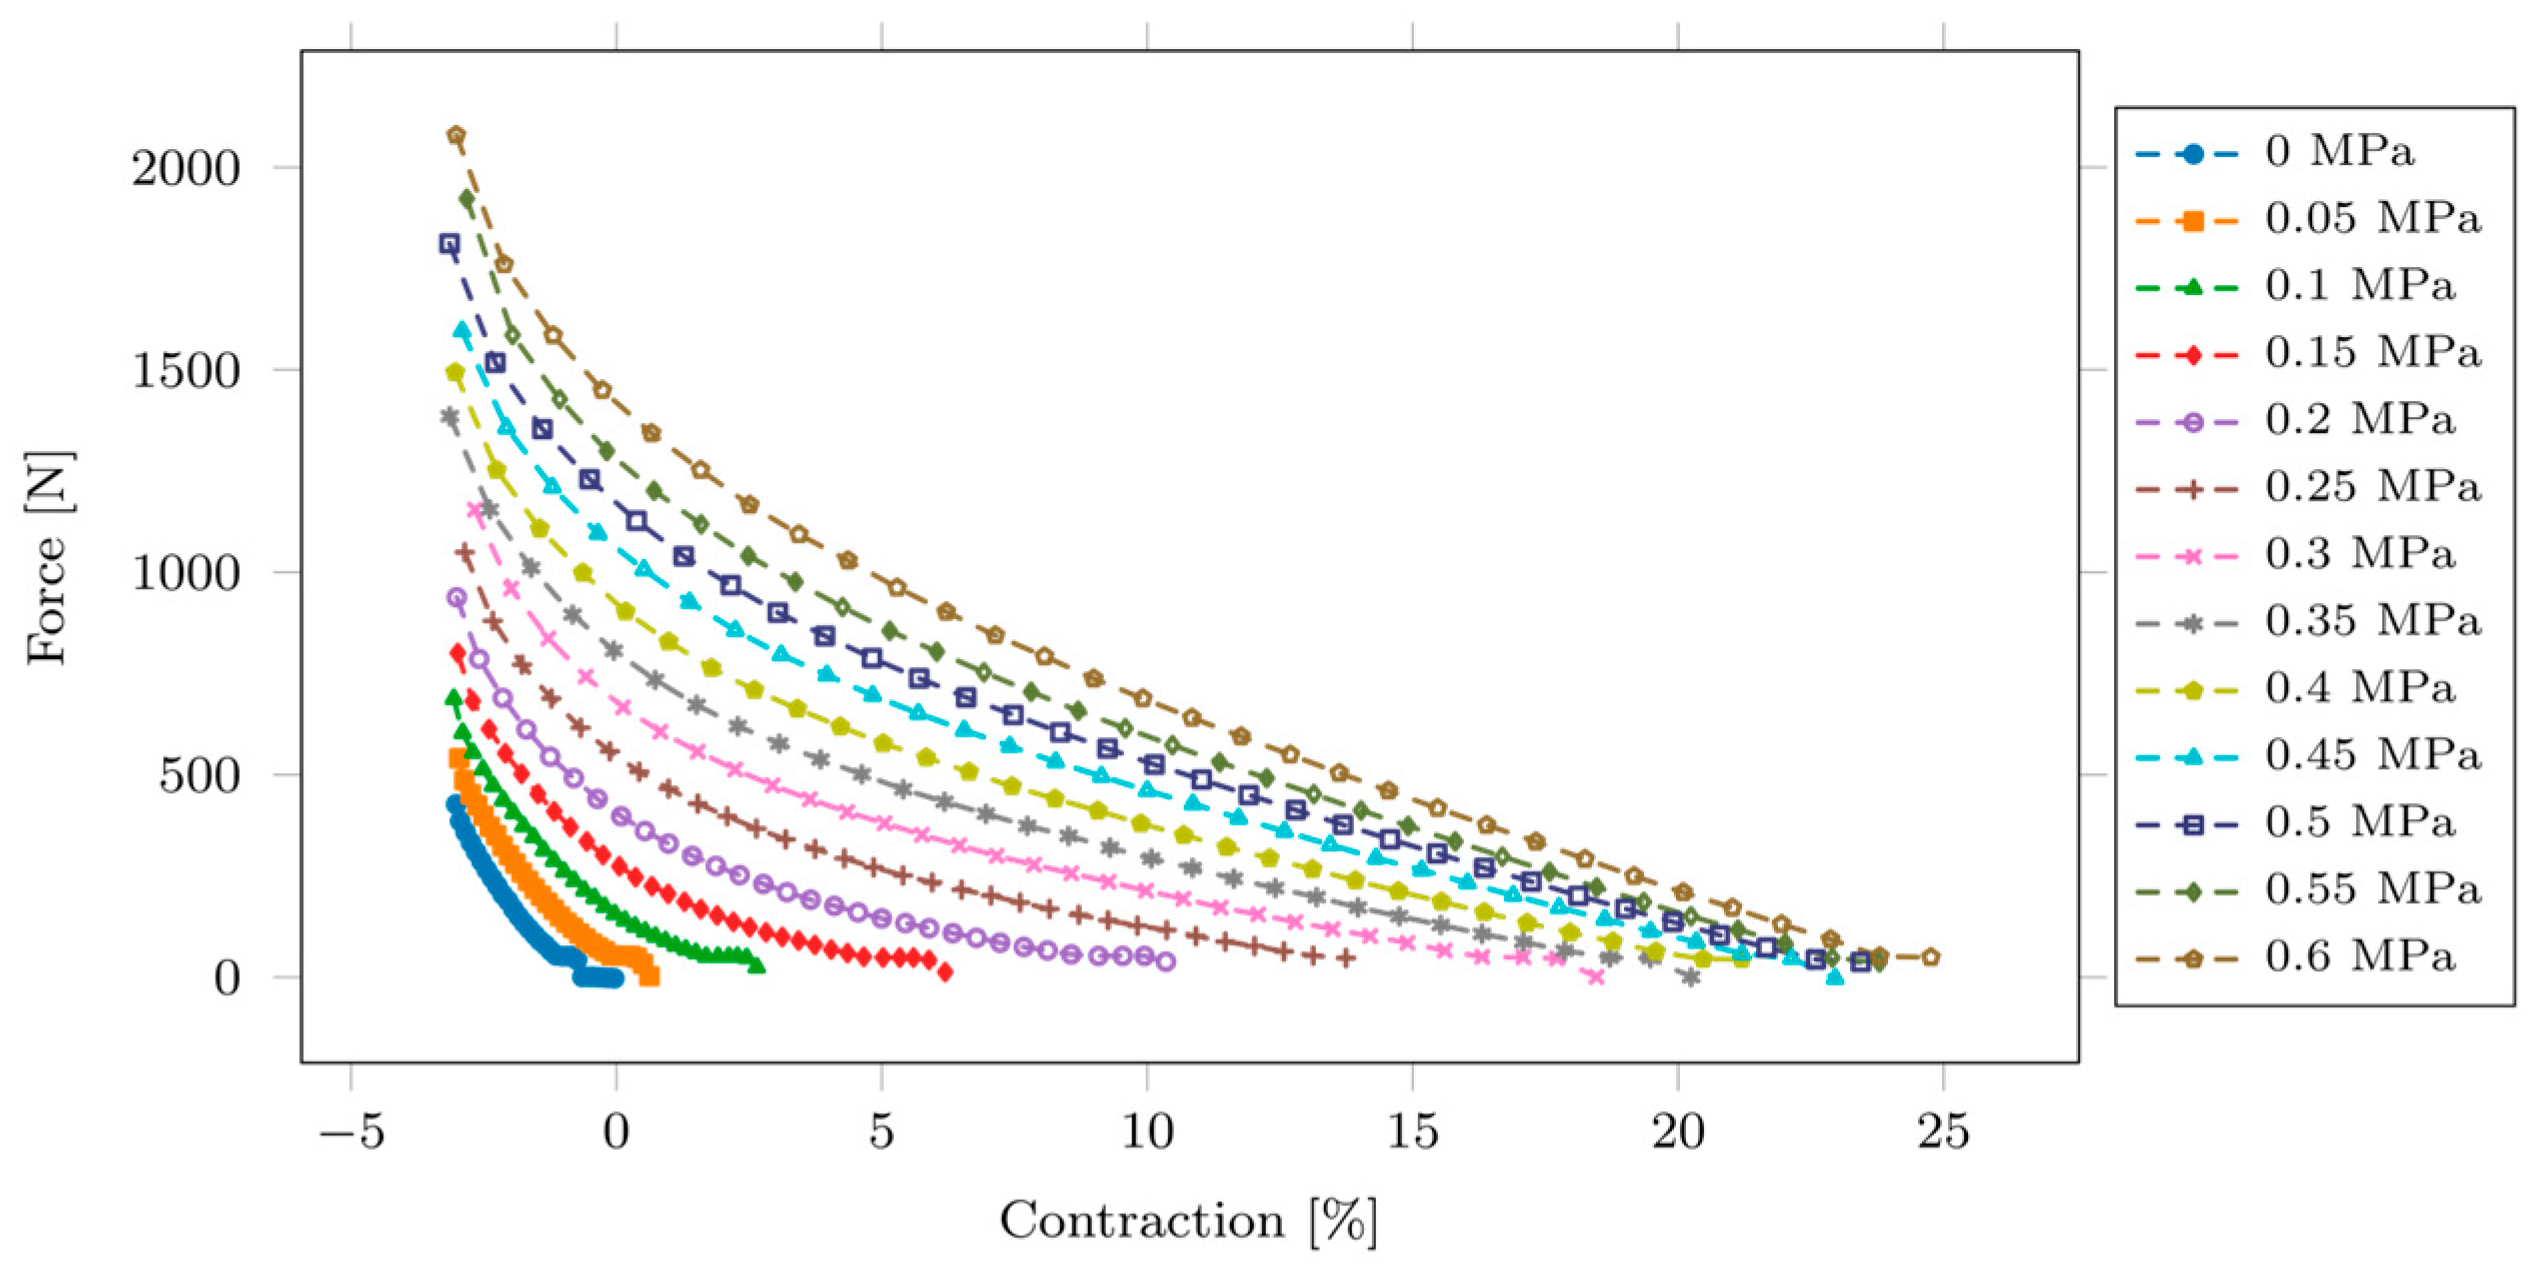
Figure 12, Figure 13, Figure 14 and Figure 15 show the corresponding force–contraction curves during the loading (expansion) path. As in the unloading case, each curve corresponds to one pressure and shows the median across five repeats.
Figure 12.
Force–contraction curves of the CPAM actuator during expansion (load cell force).
Figure 13.
Force–contraction curves of the CPAM actuator during expansion (excitation force).
Figure 14.
Force–contraction curves of the DMSP actuator during expansion (load cell force).
Figure 15.
Force–contraction curves of the DMSP actuator during expansion (excitation force).
Both muscles exhibit clear hysteresis: for a given contraction, the force on the expansion branch is higher than on the contraction branch at the same pressure. The general shape of the loops is similar for the two actuators, but some differences emerge:
- The CPAM maintains higher force levels than the commercial muscle over most of the expansion branch at lower pressures.
- The difference between loading and unloading curves is more pronounced at higher pressures, which is consistent with larger internal stresses and frictional effects at higher loads.
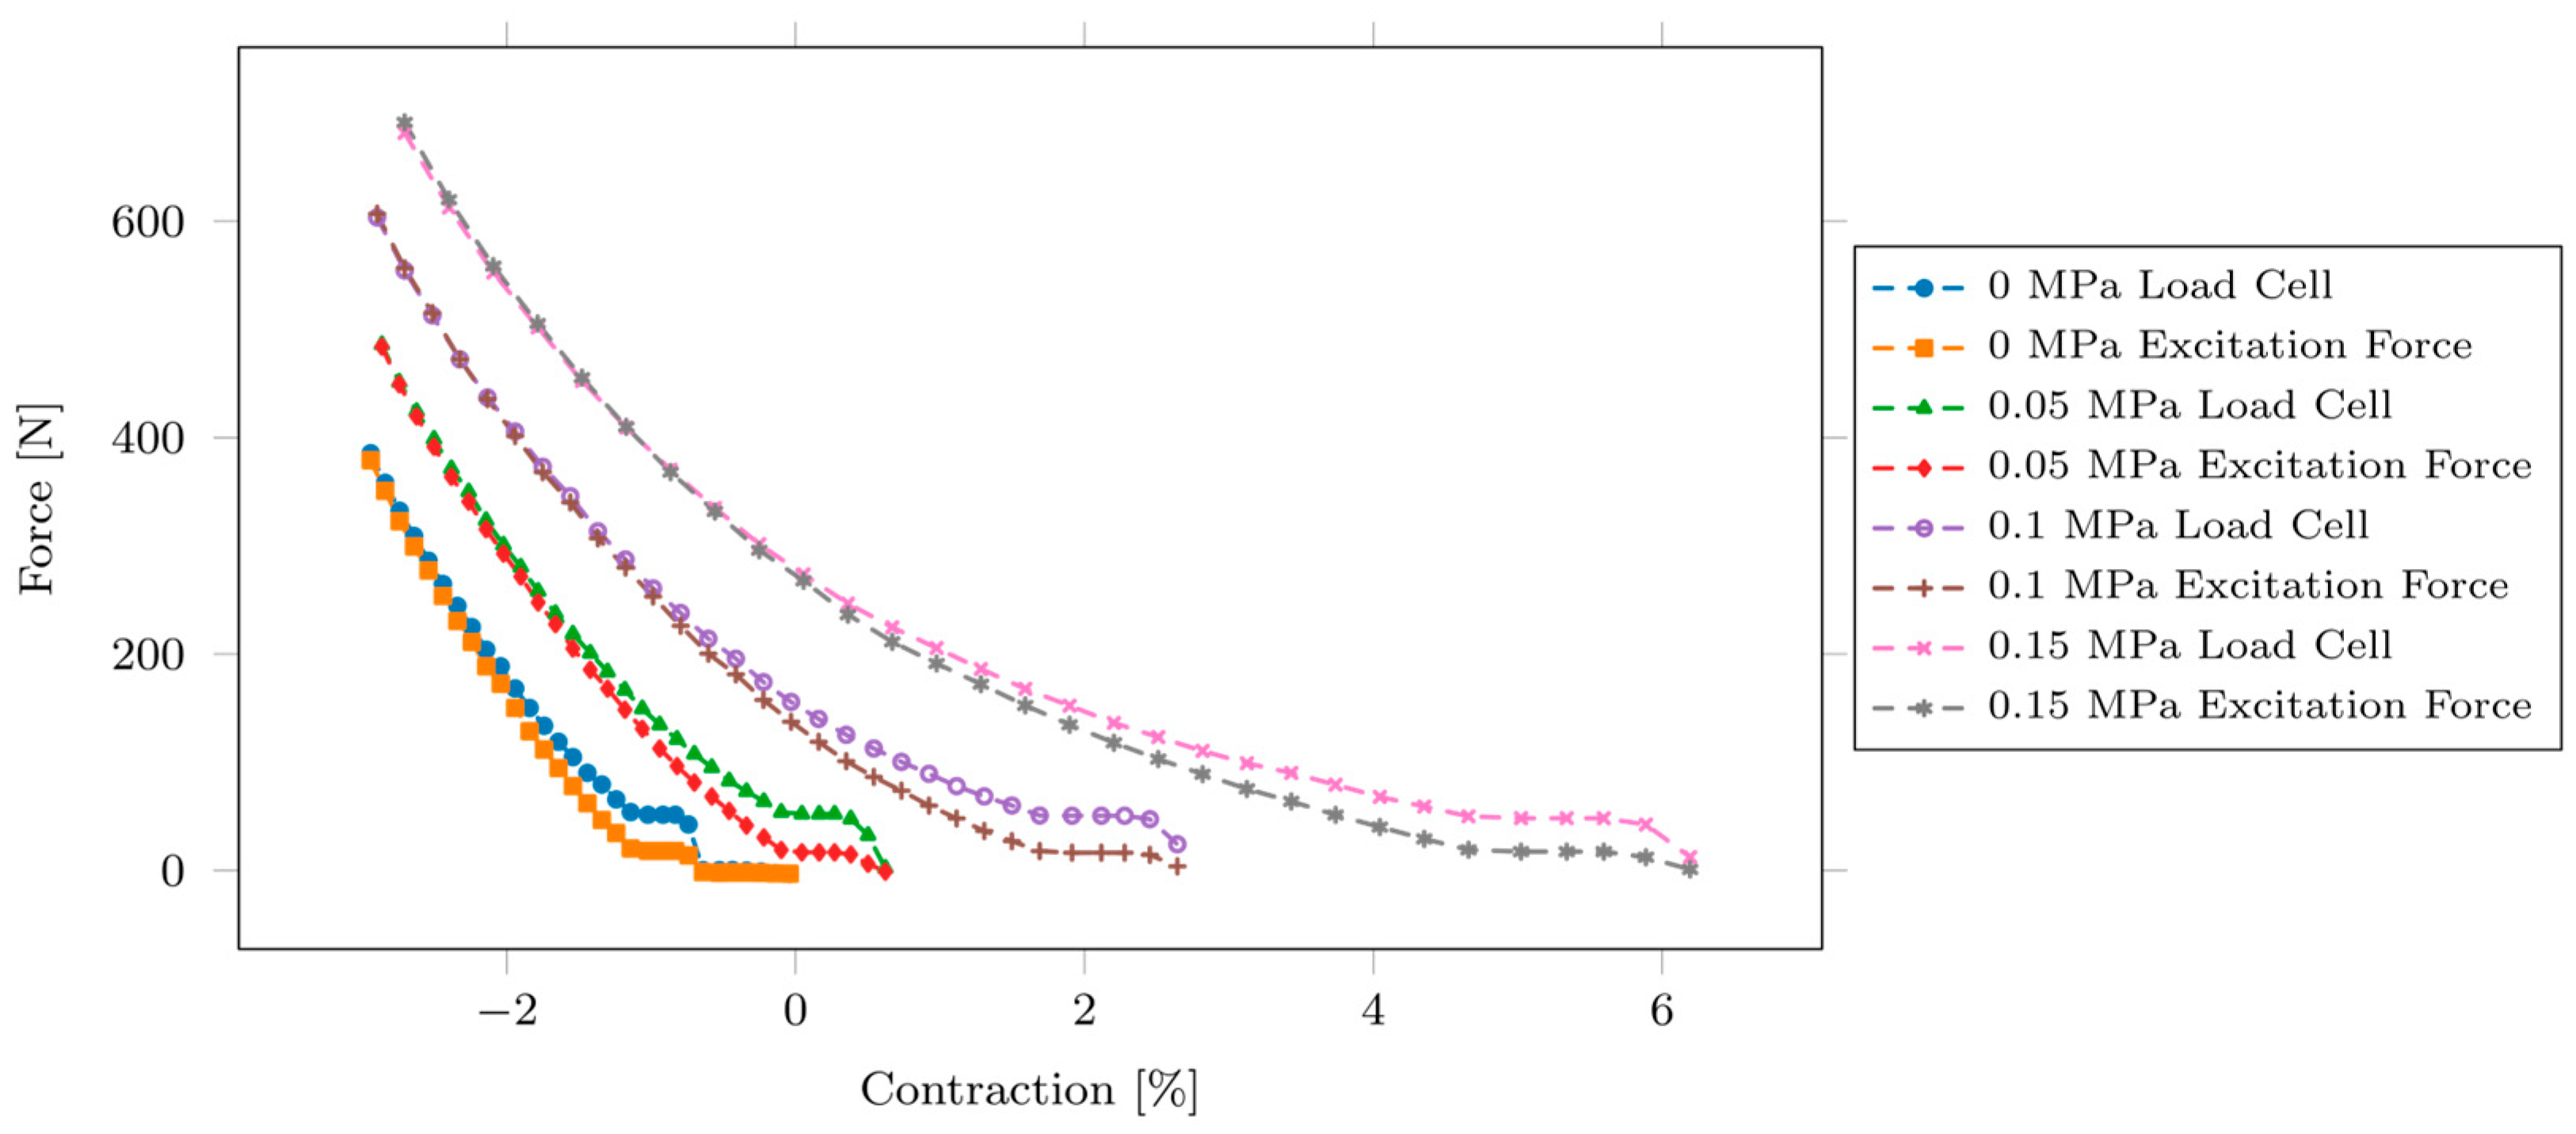
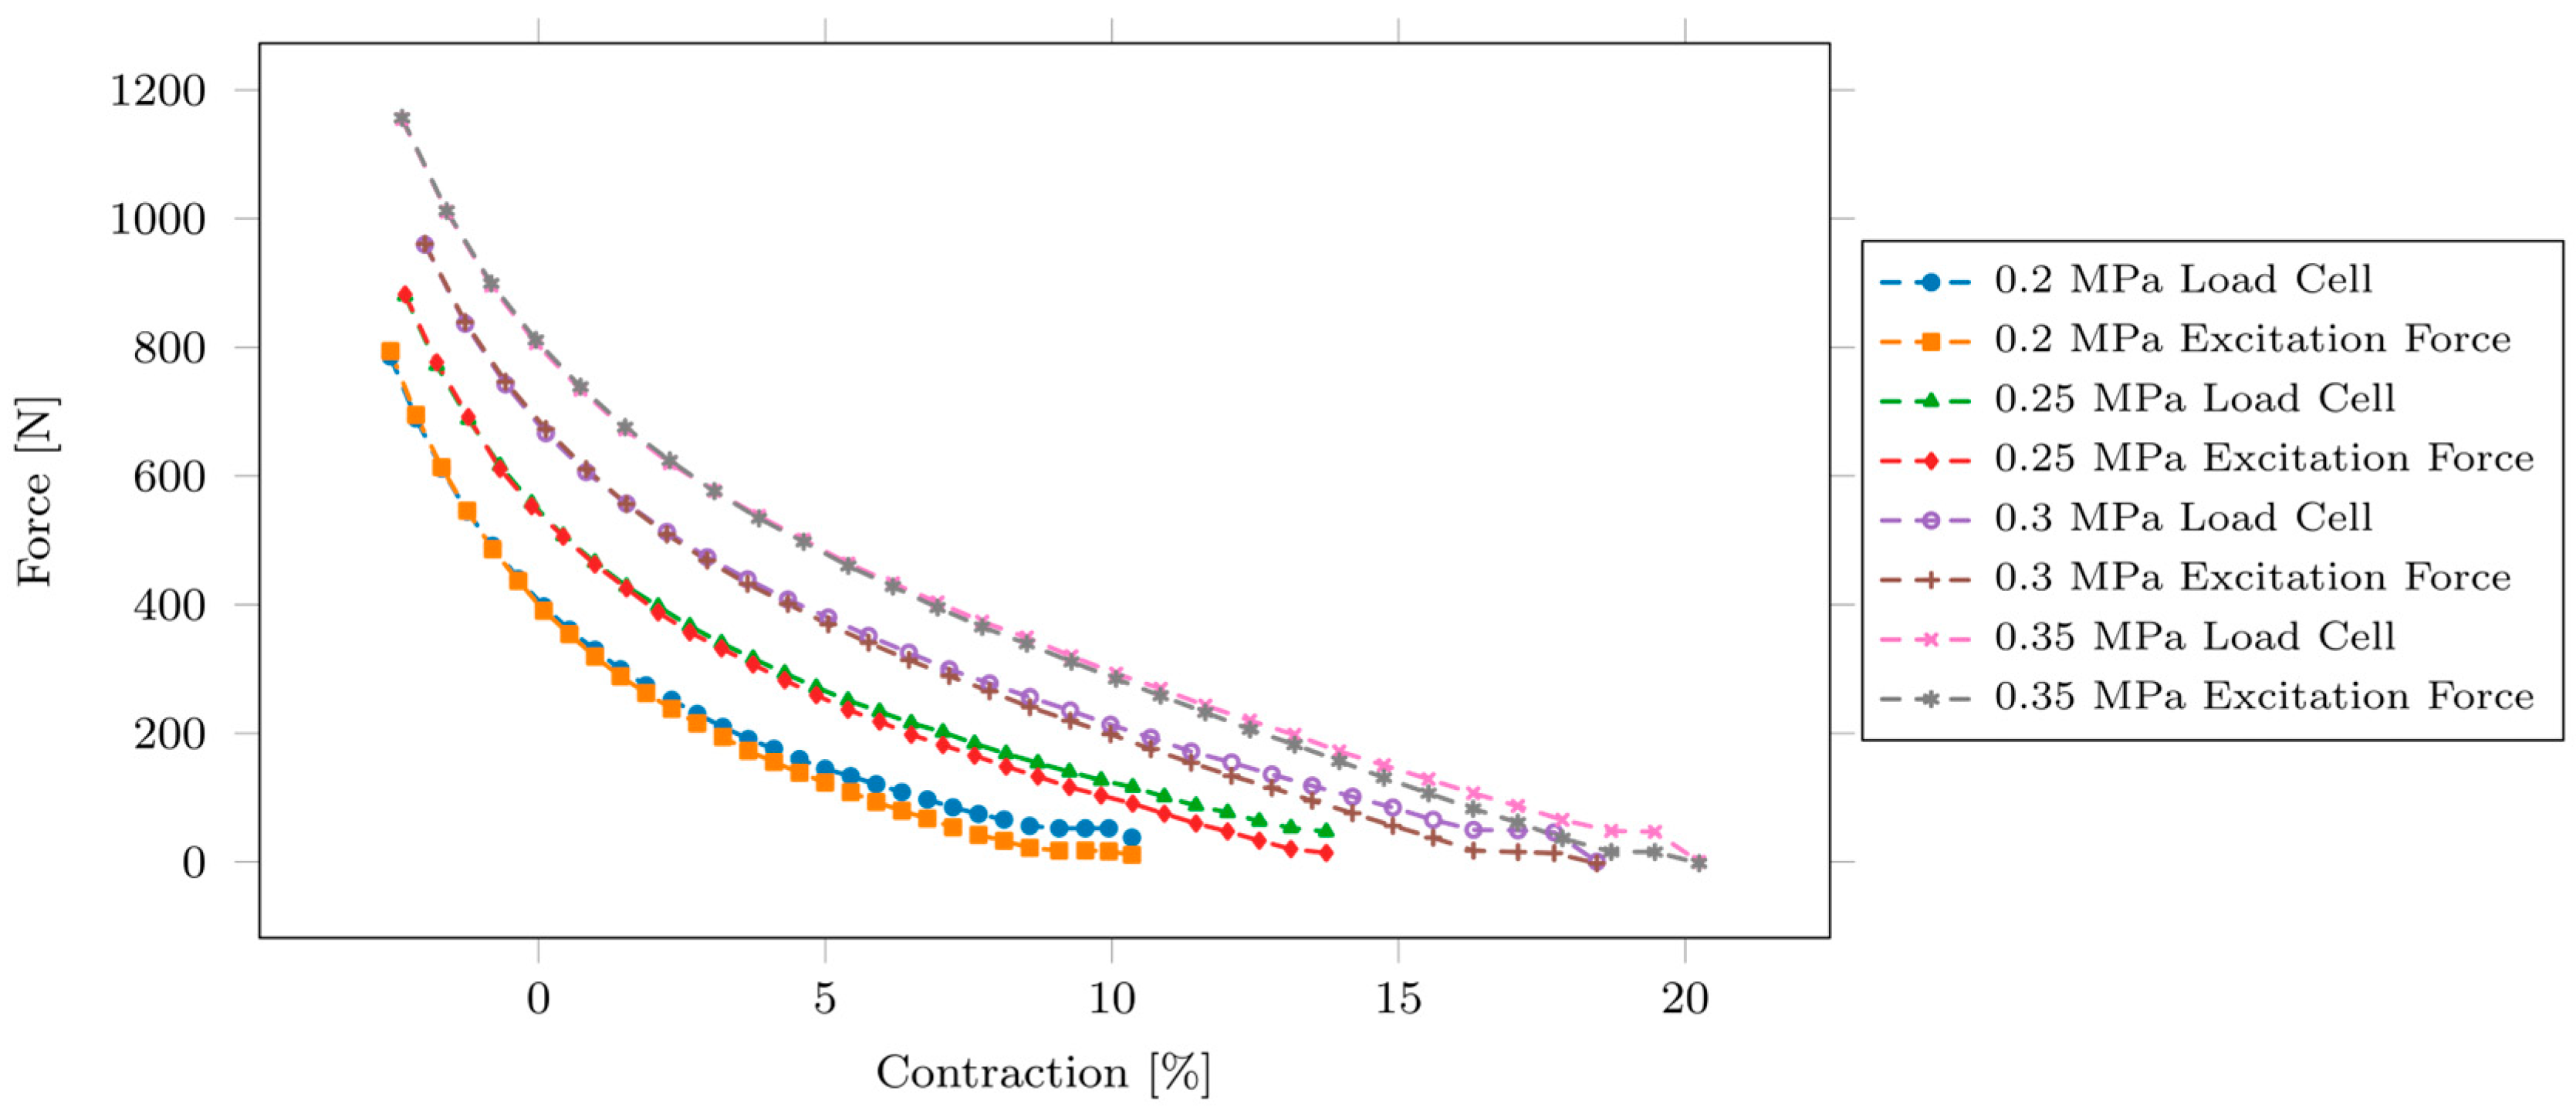
In the commercial DMSP-20-200N muscle, the loading branch when reading the measured force often exhibits a small additional loop or kink on the expansion side that is absent or much less pronounced in the CPAM. This feature is accompanied by a larger difference between the excitation force Fexcitation and the measured muscle force Fmeasured along the unloading branch, indicating that a non-negligible part of the input work is dissipated or stored internally in the commercial muscle rather than transmitted to the load. In contrast, the CPAM shows a more regular single-loop behavior with a smaller Fexcitation–Fmeasured mismatch on the expansion side.
Repeat-to-repeat variability is low, and the loops are well reproducible over the five cycles for both muscles.
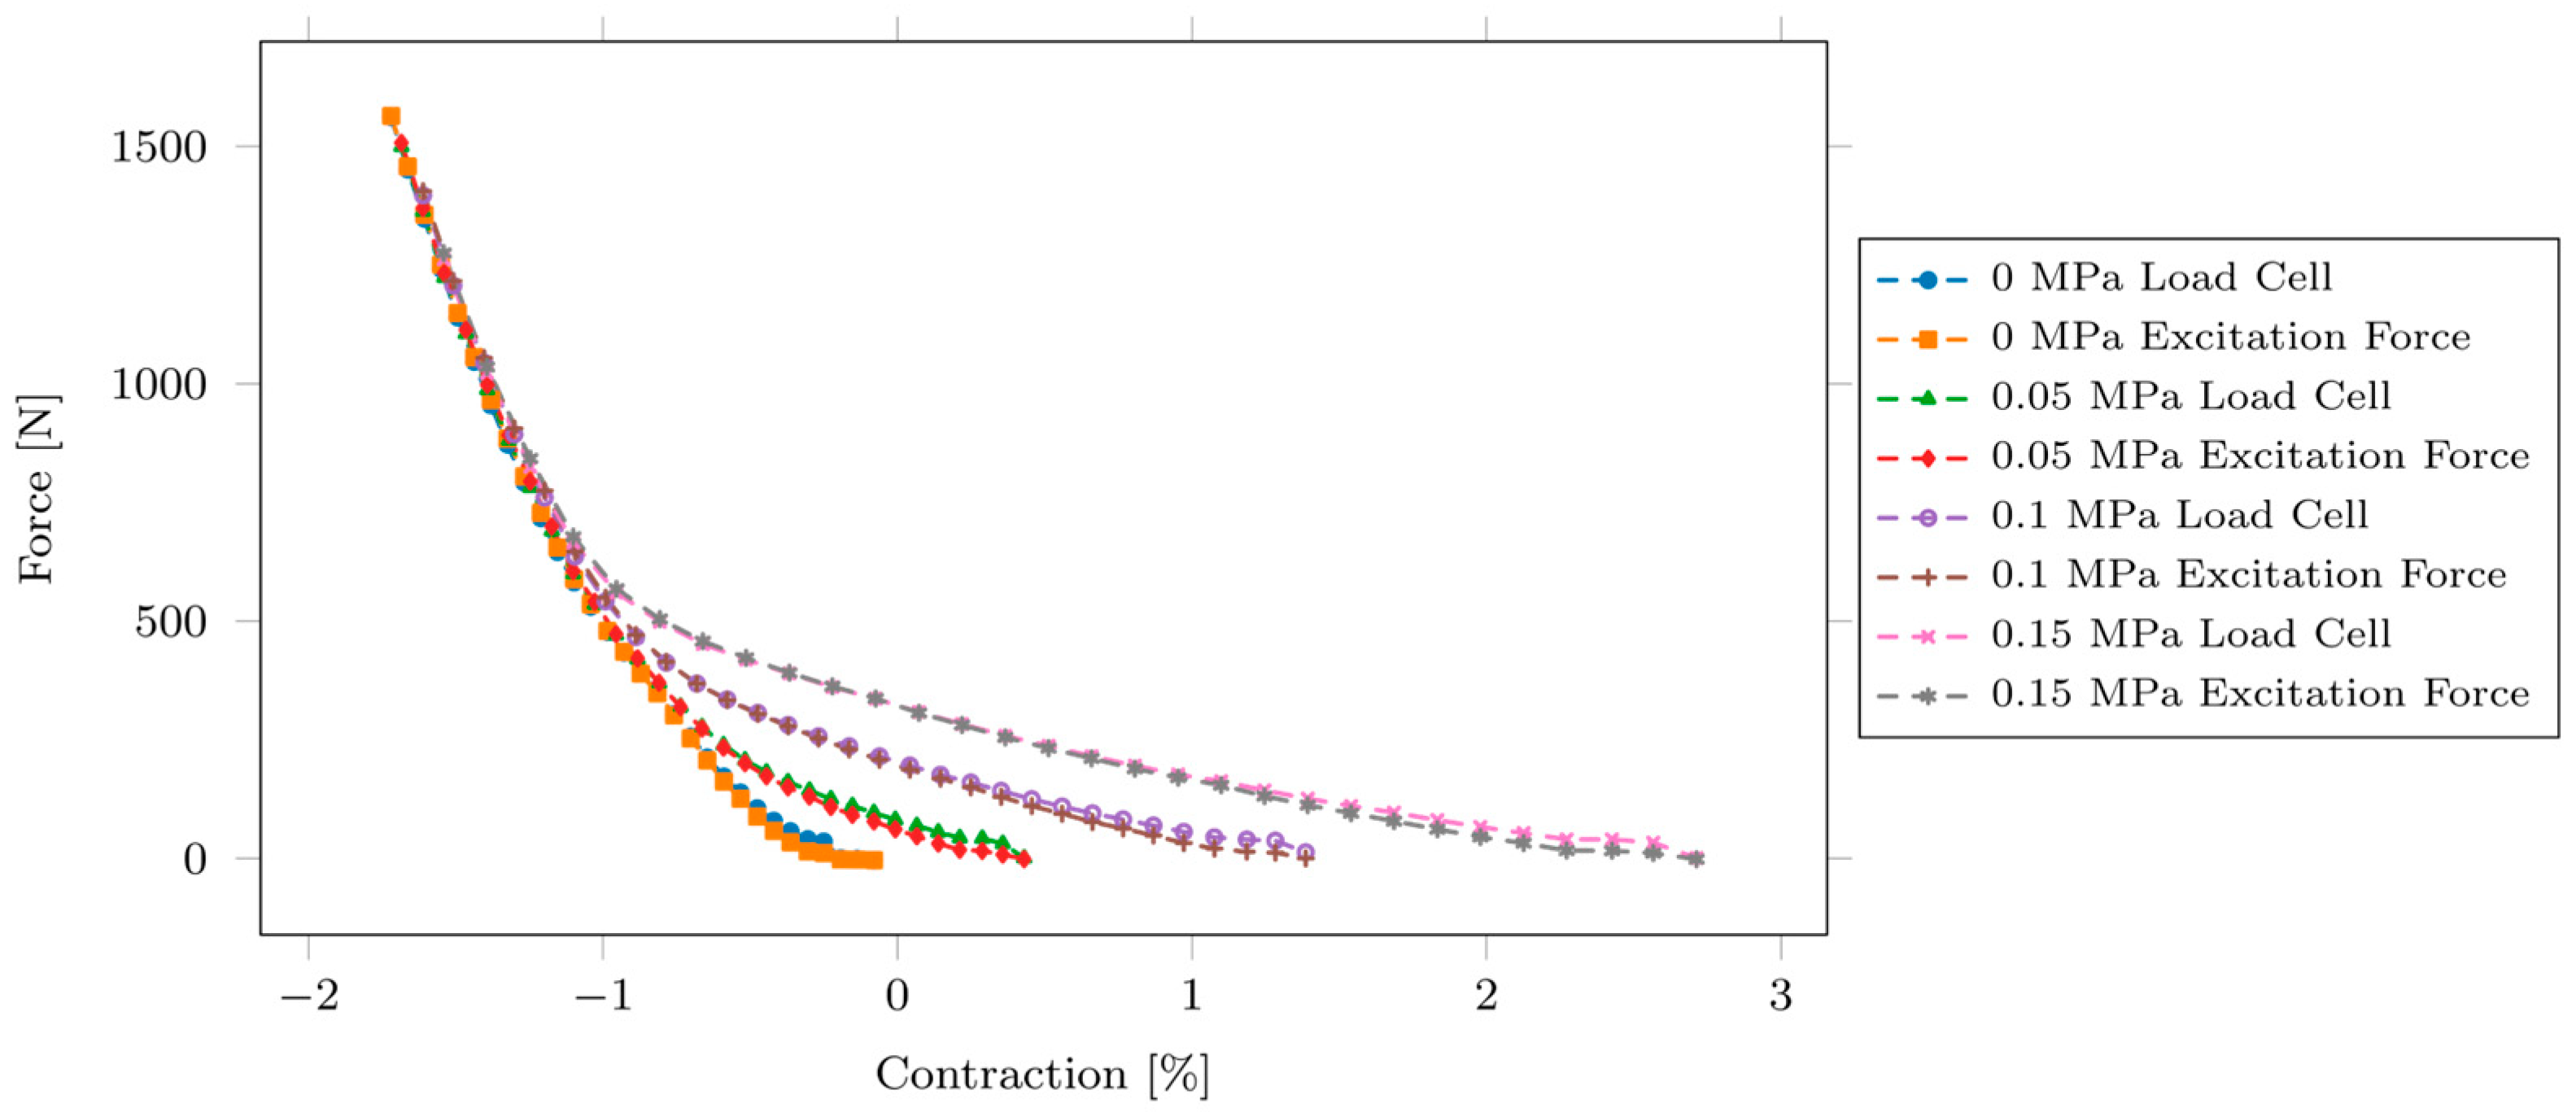
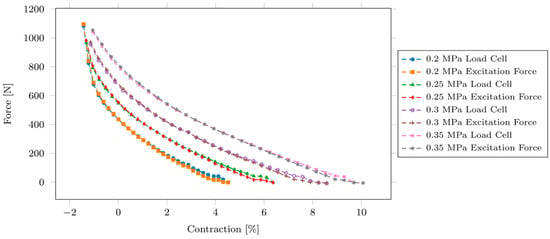
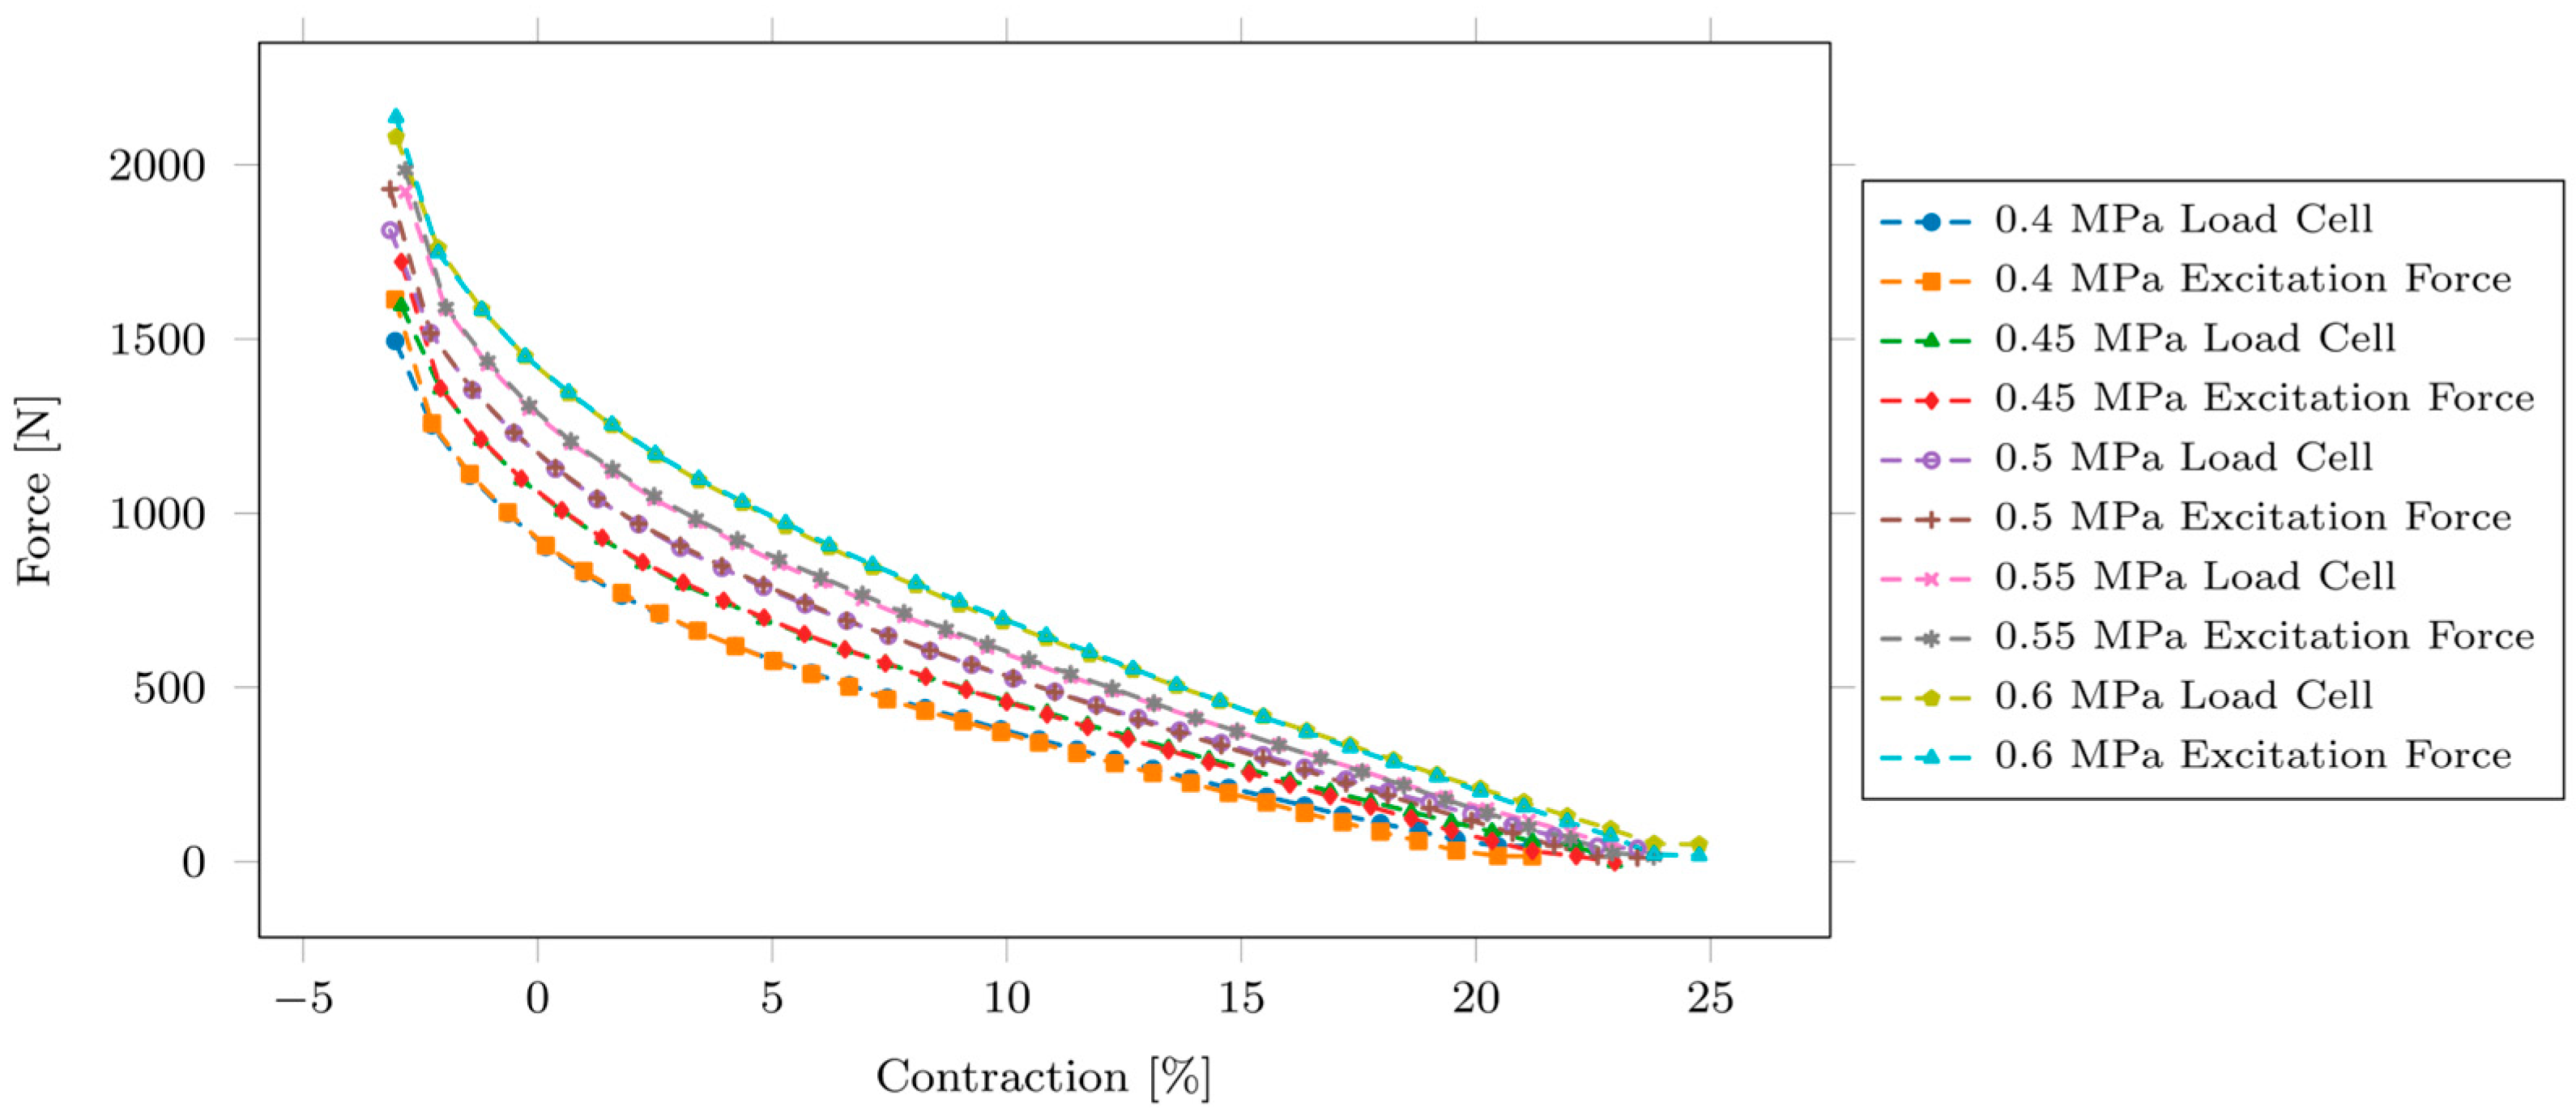
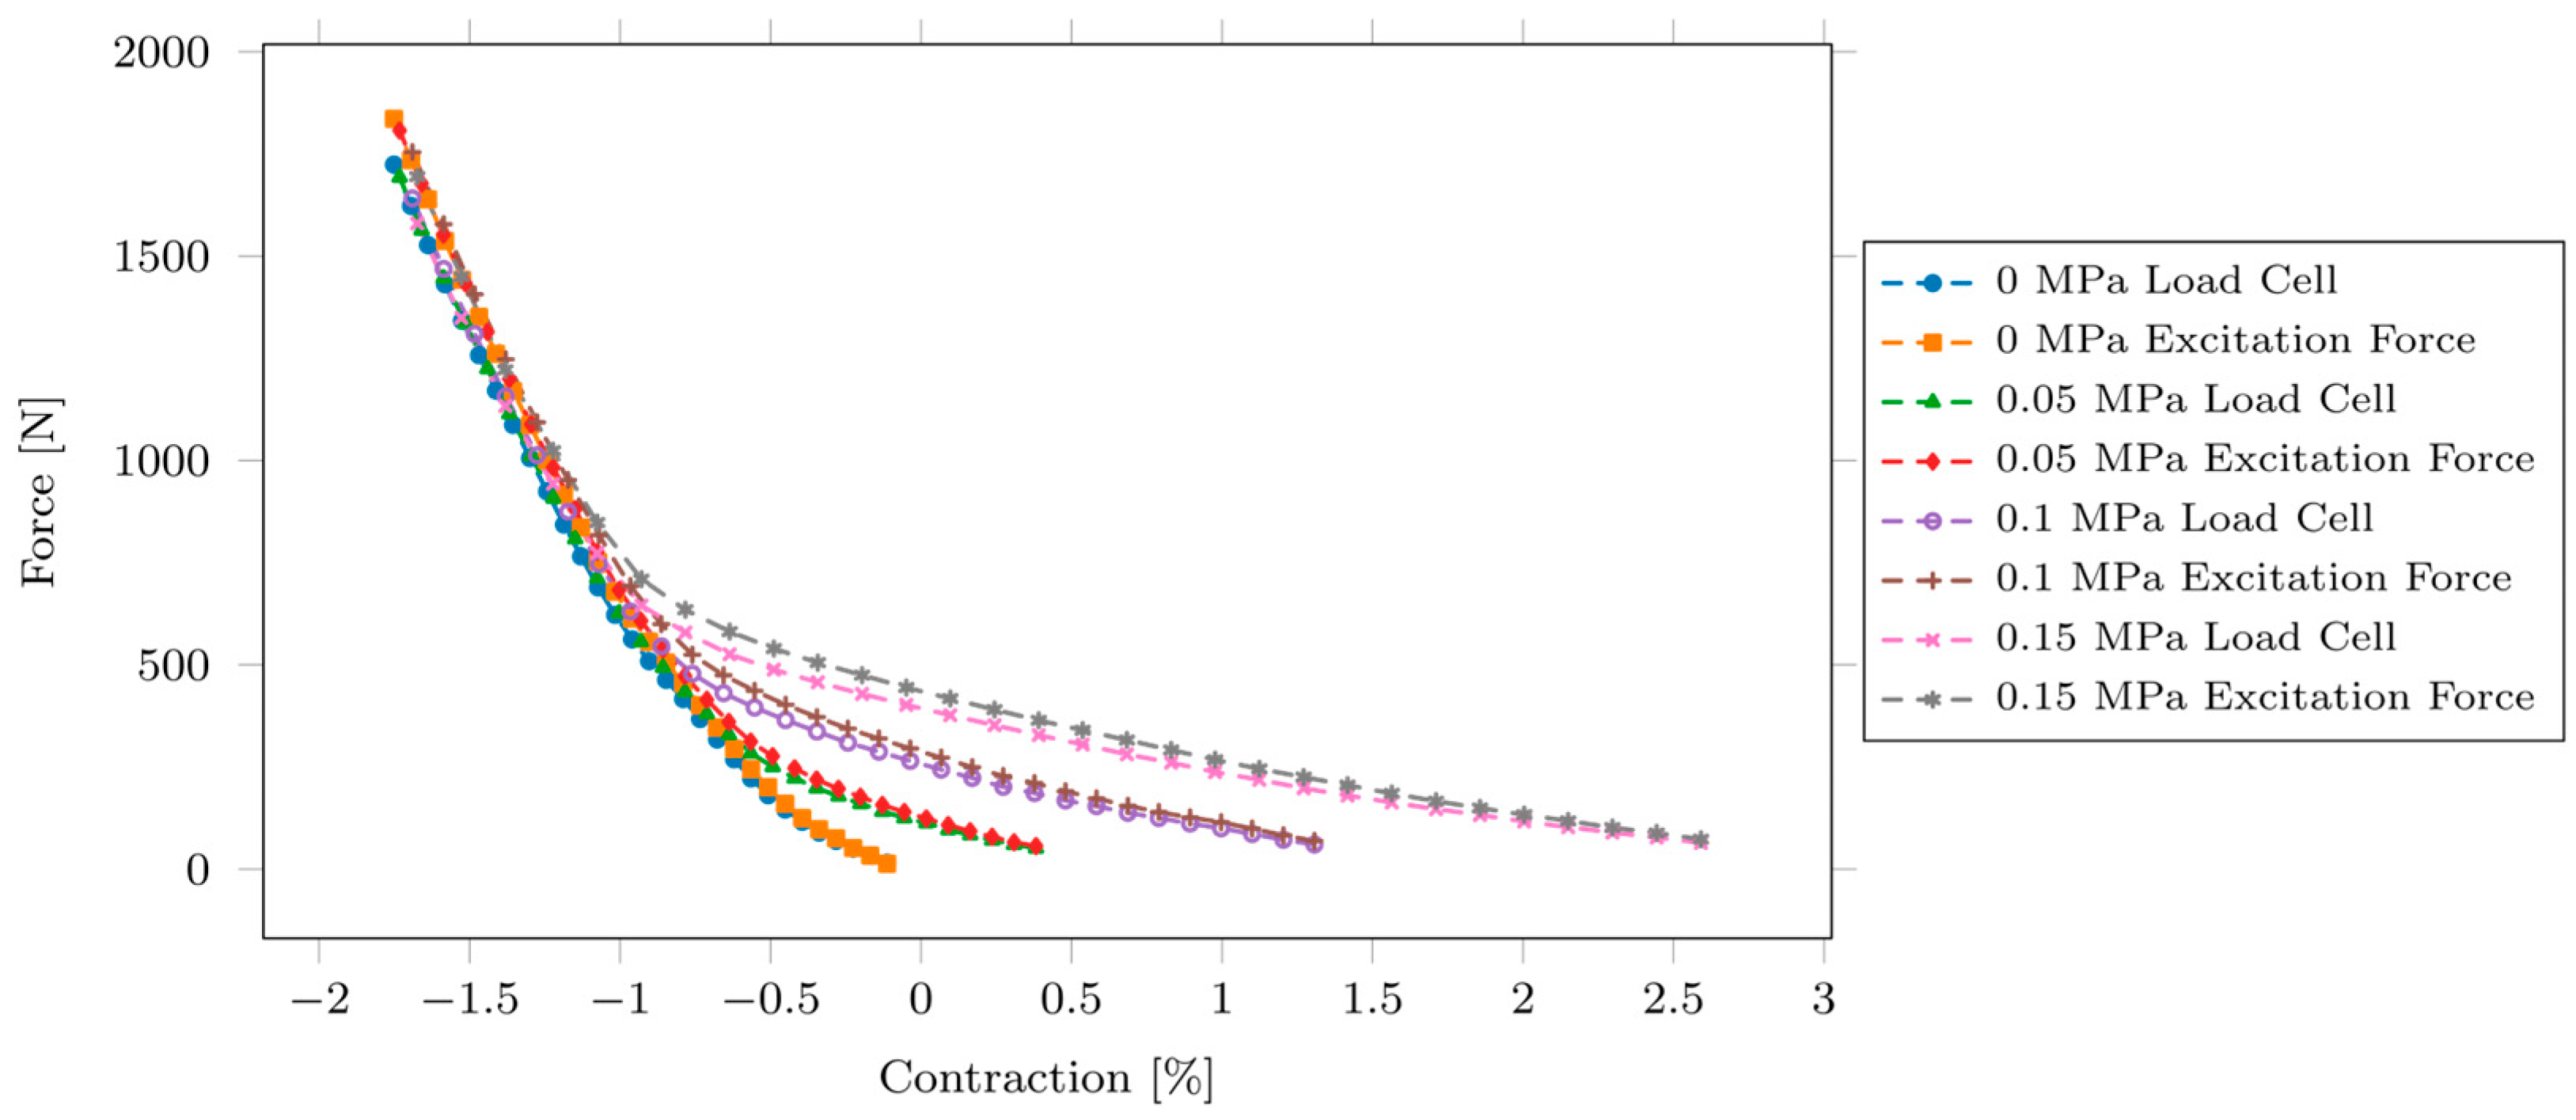
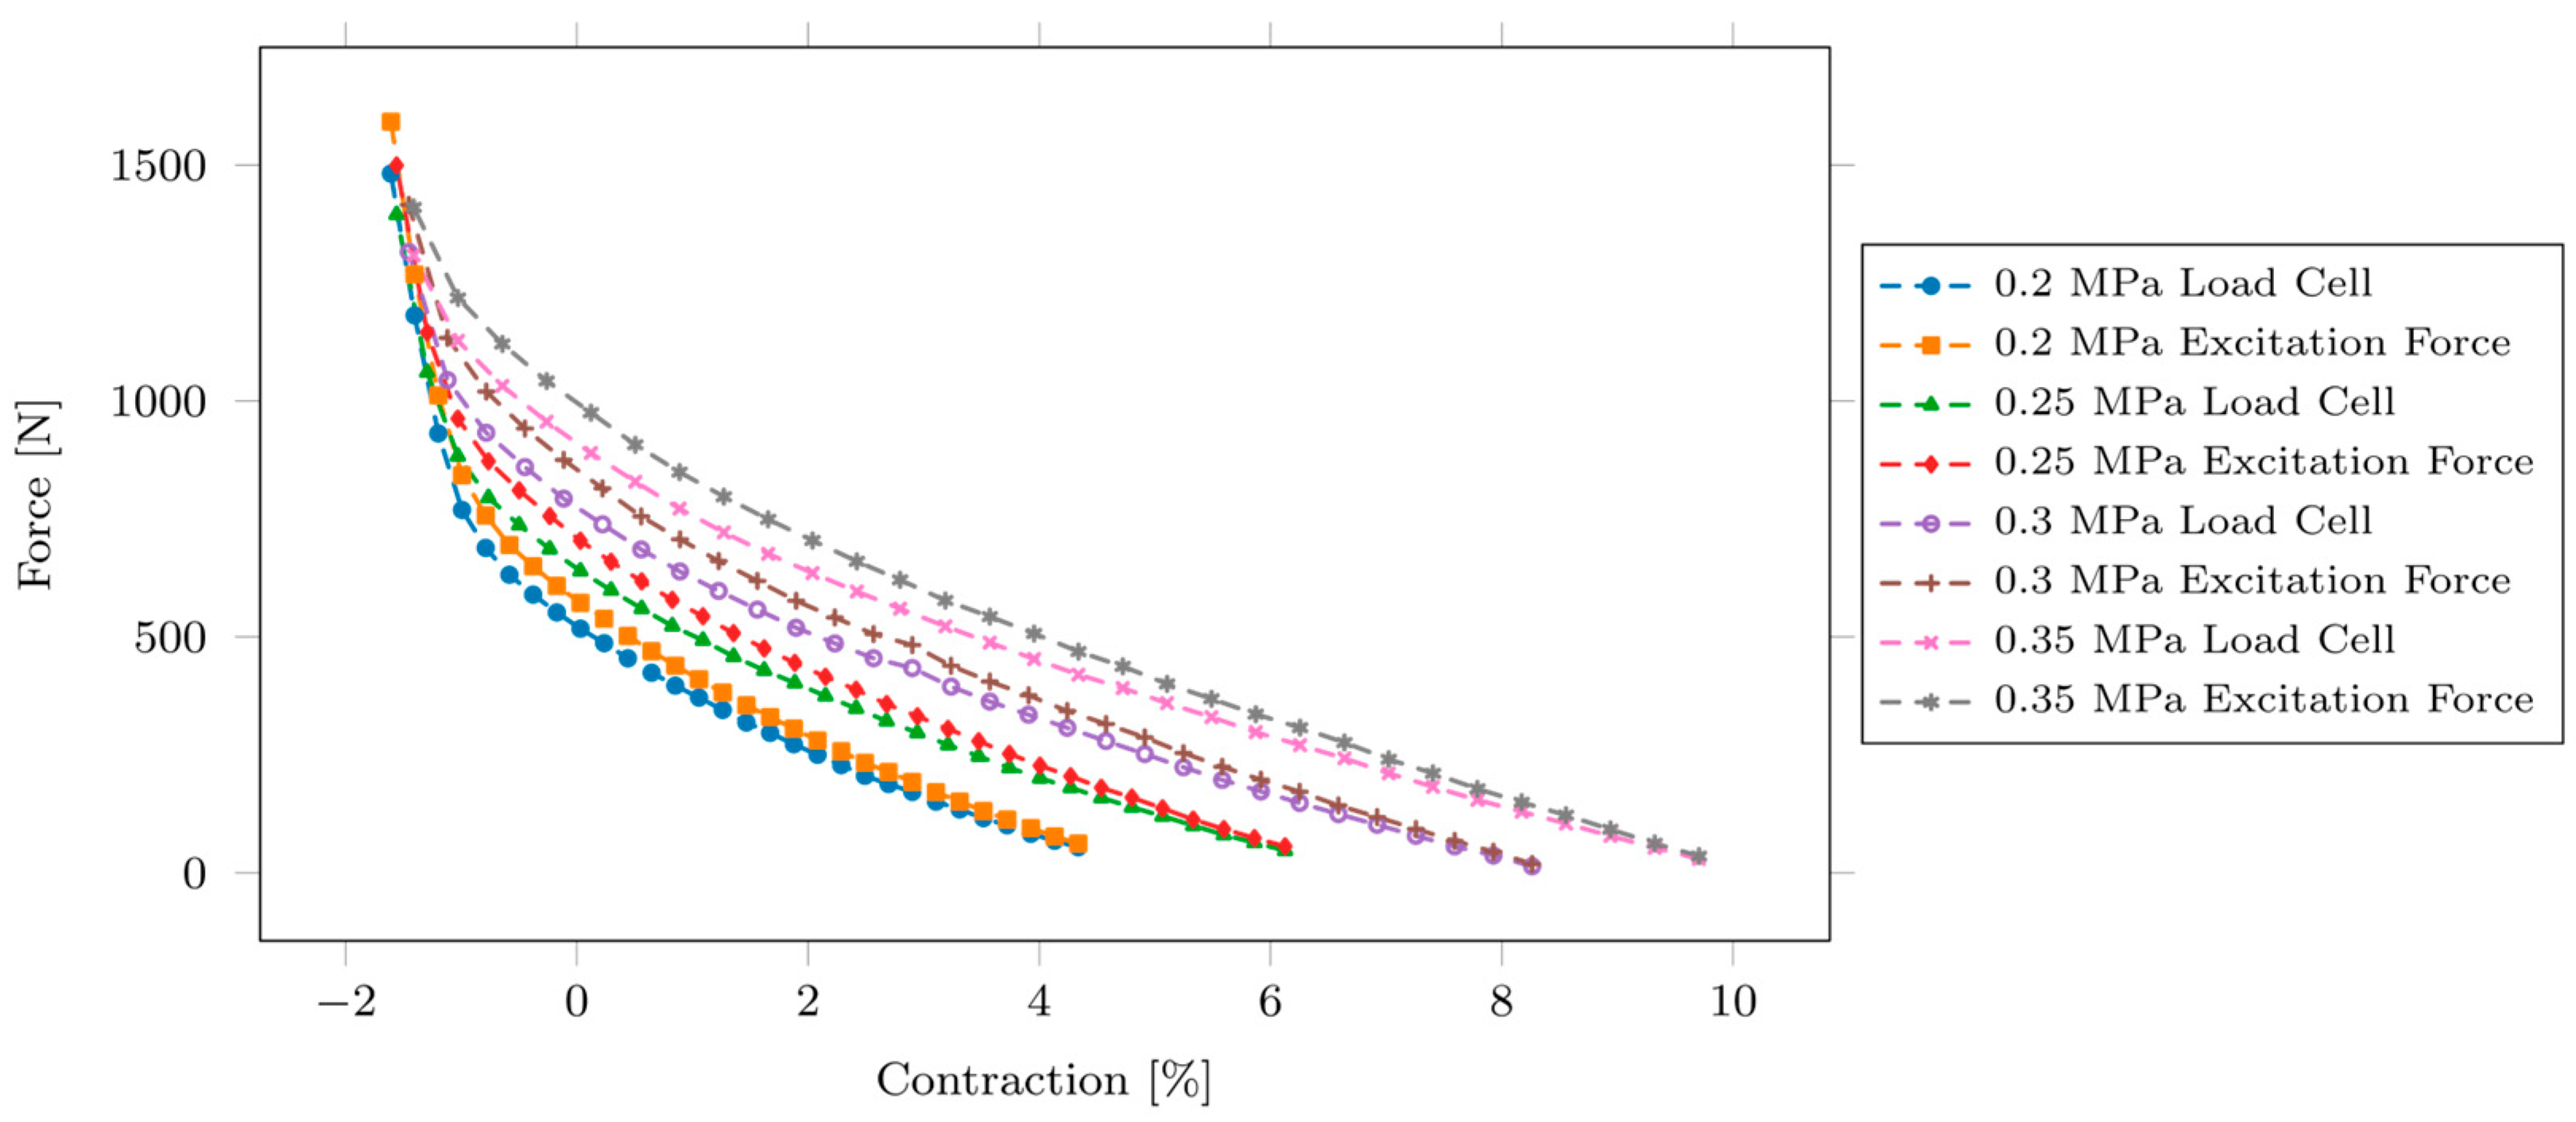
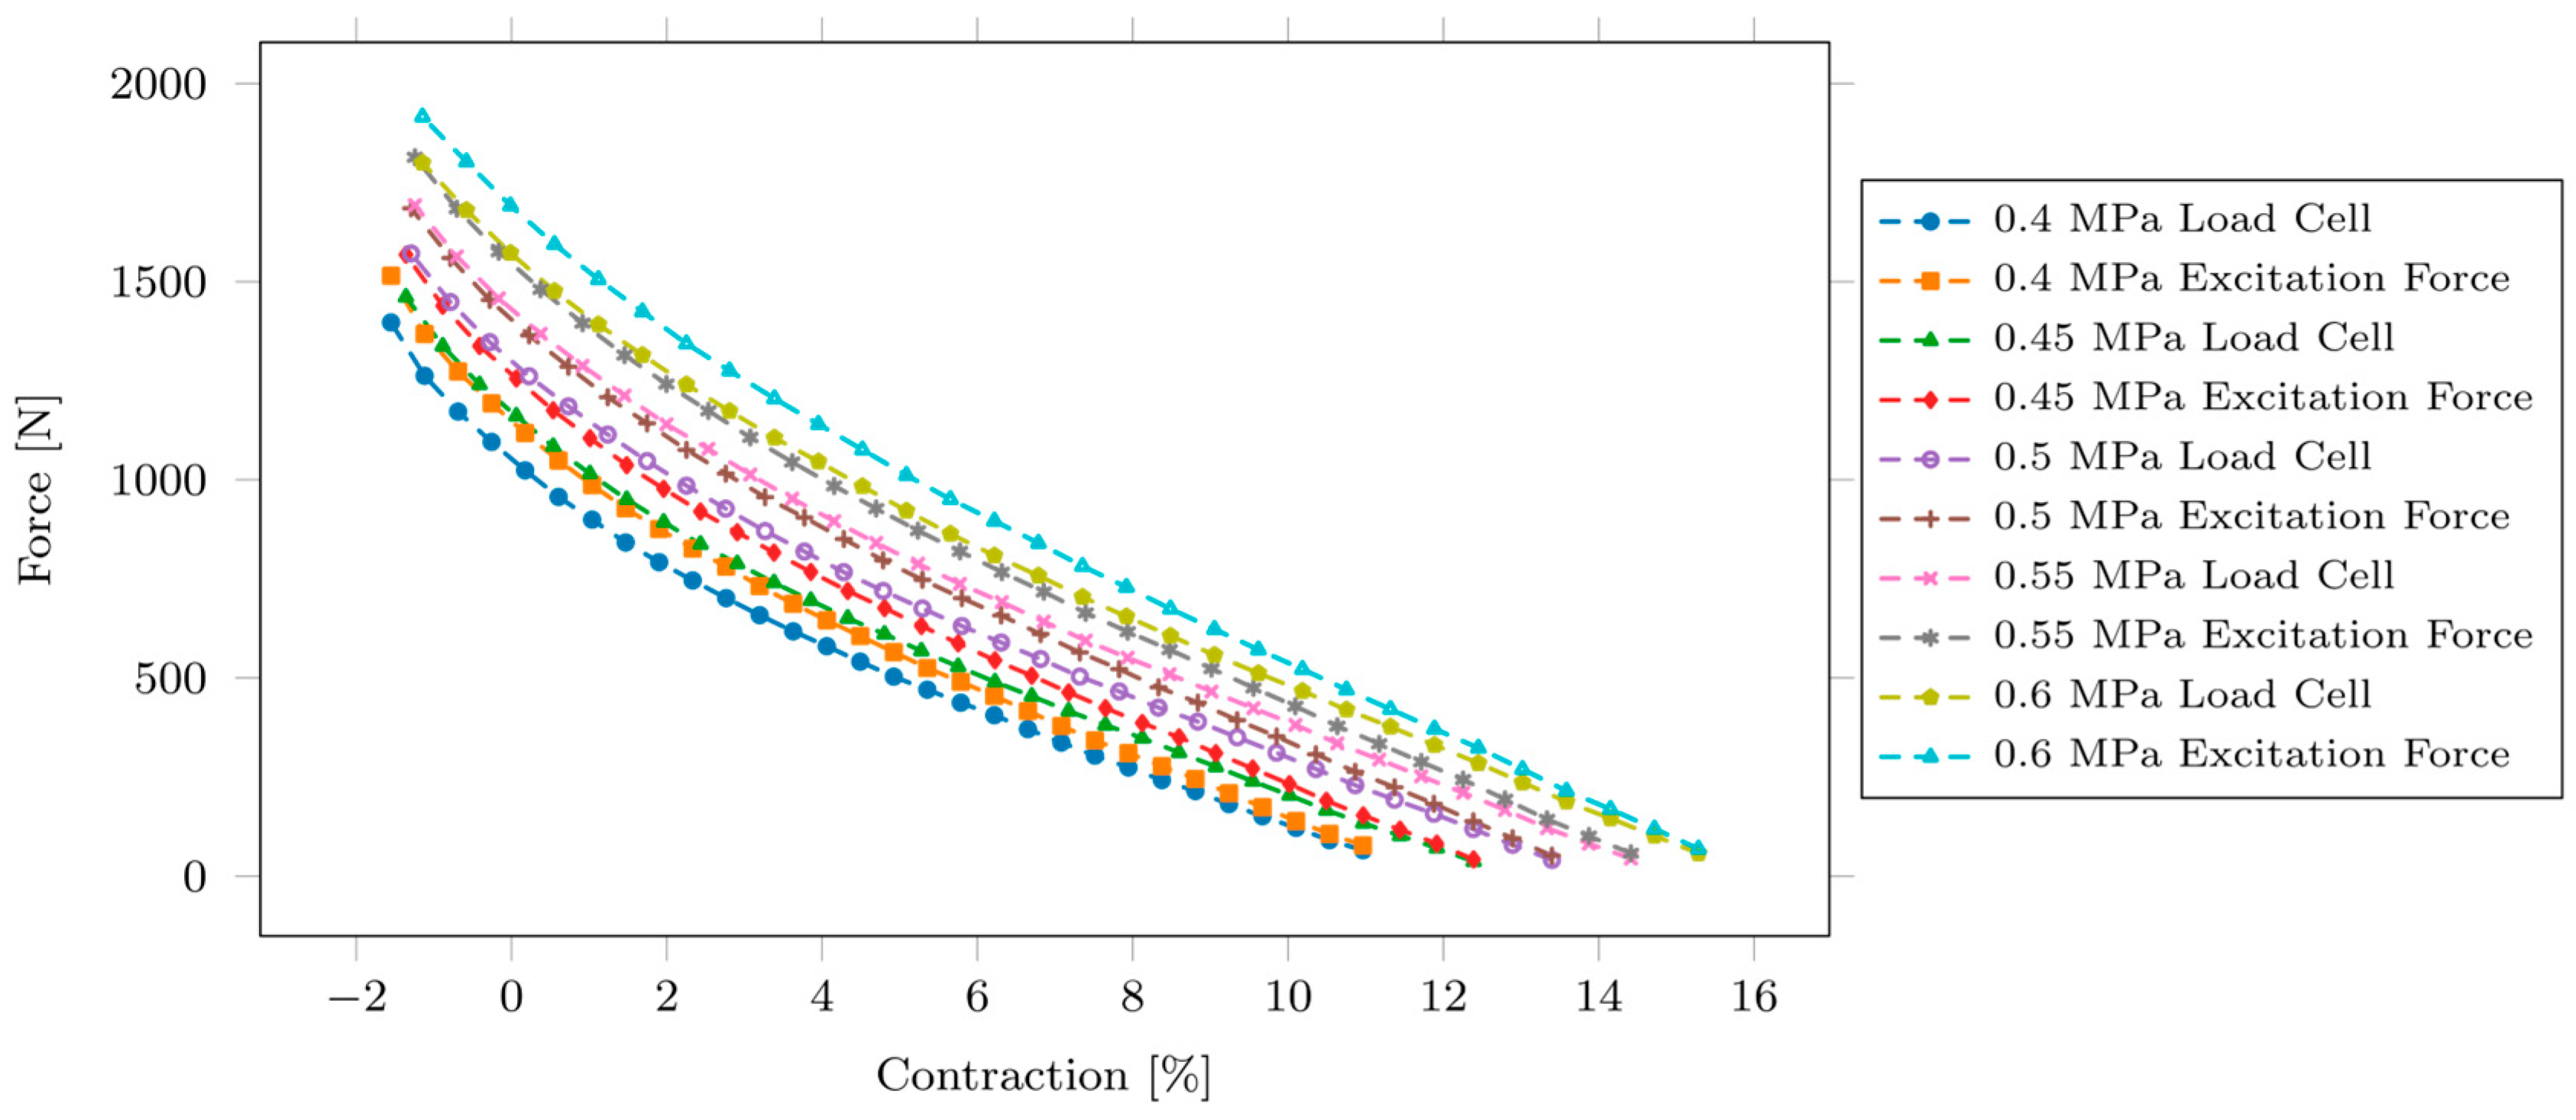
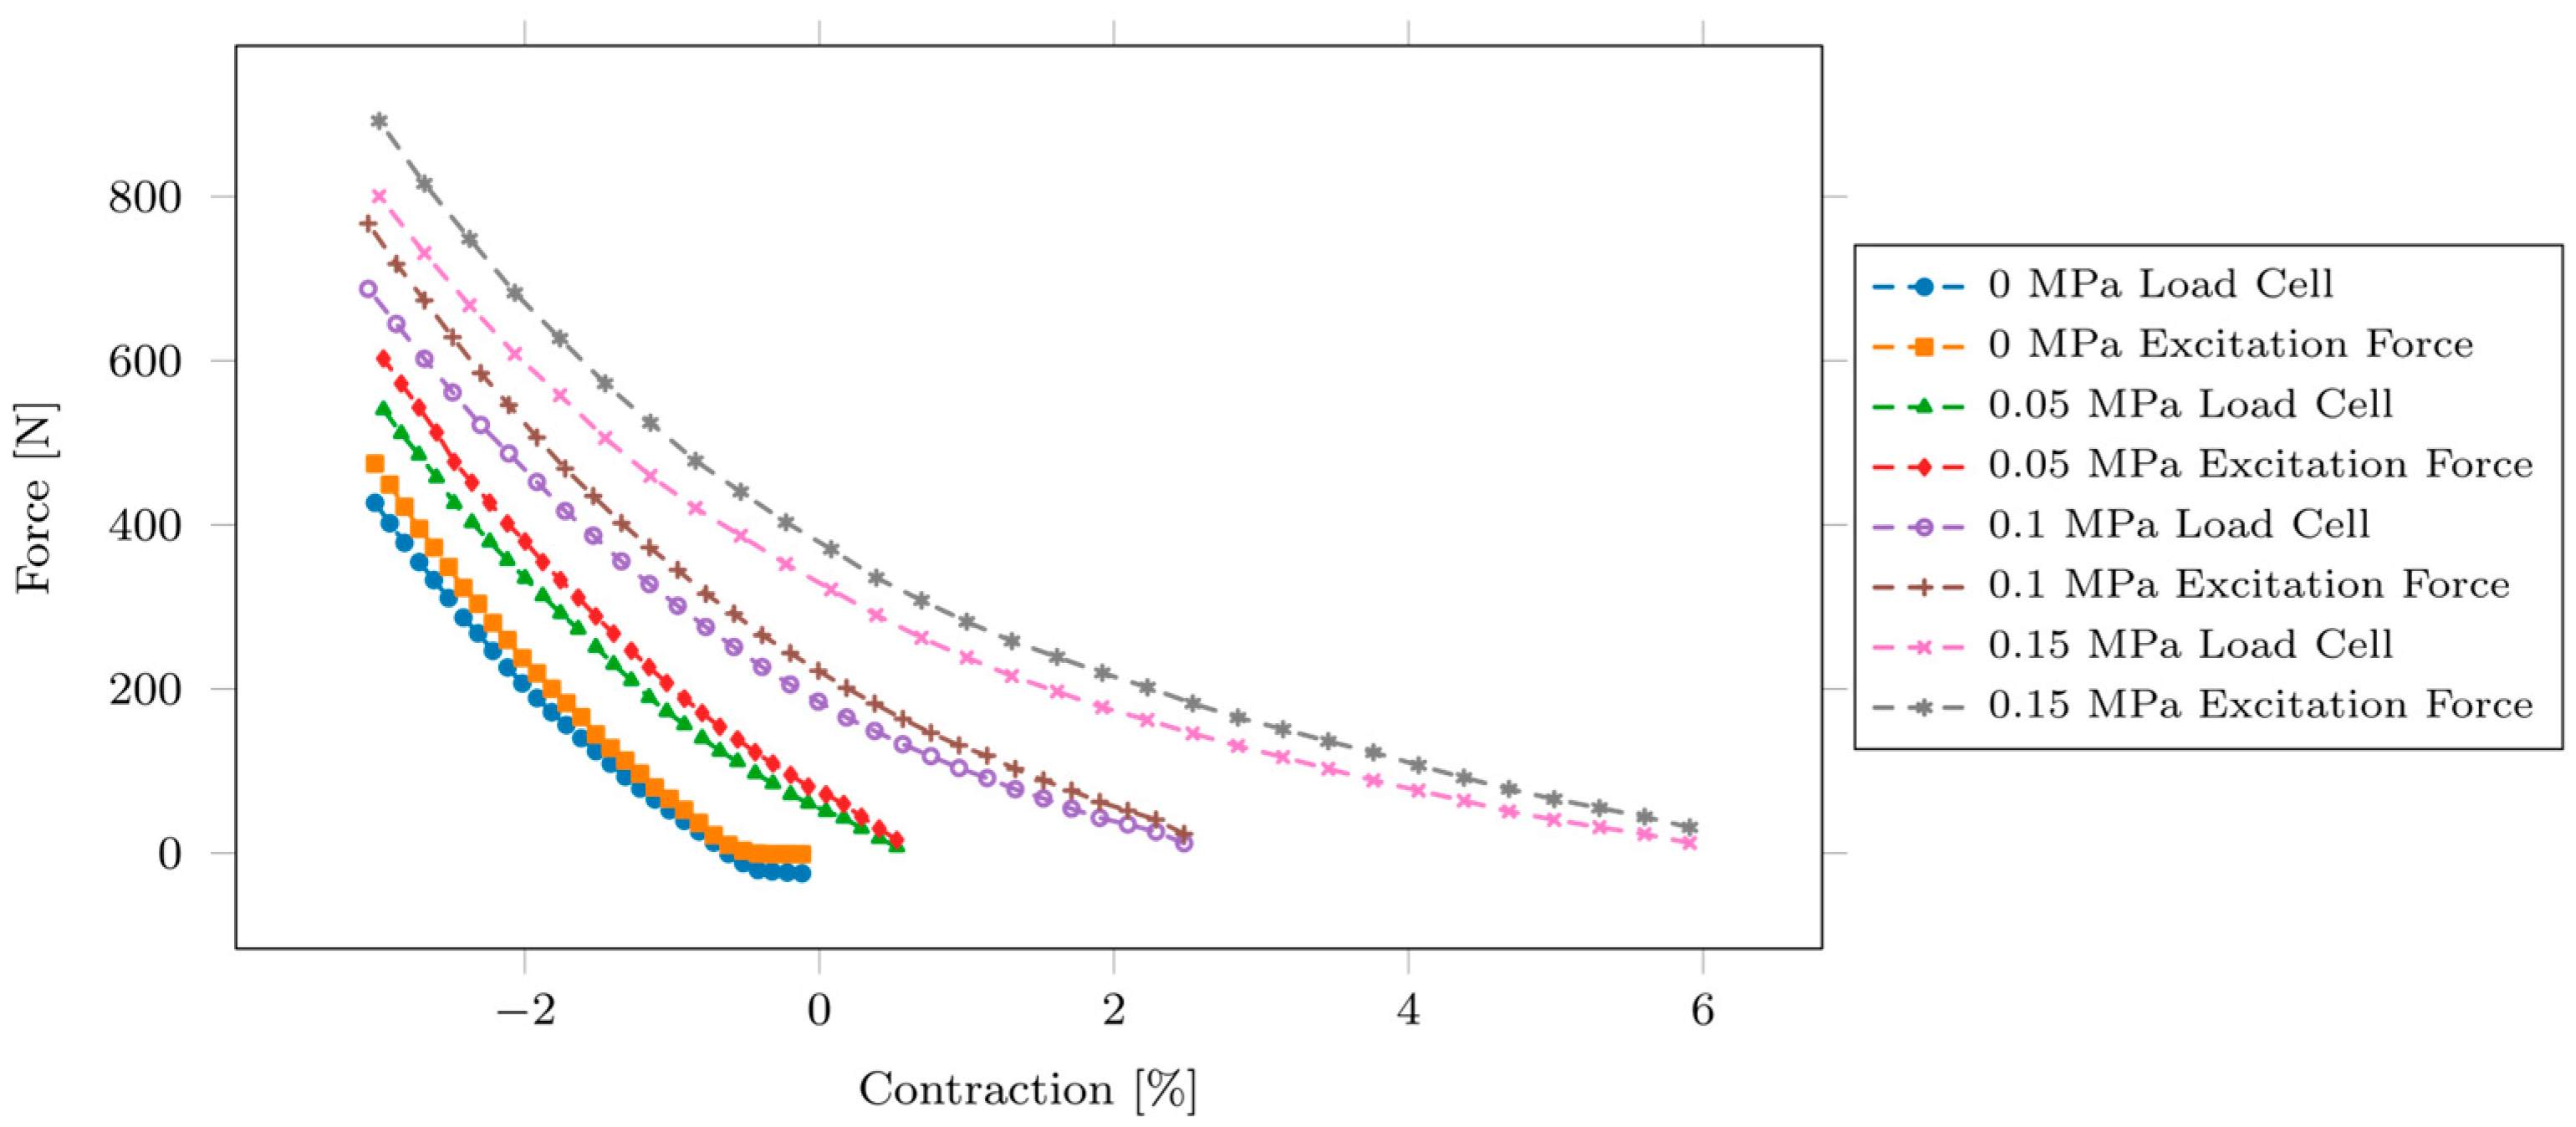
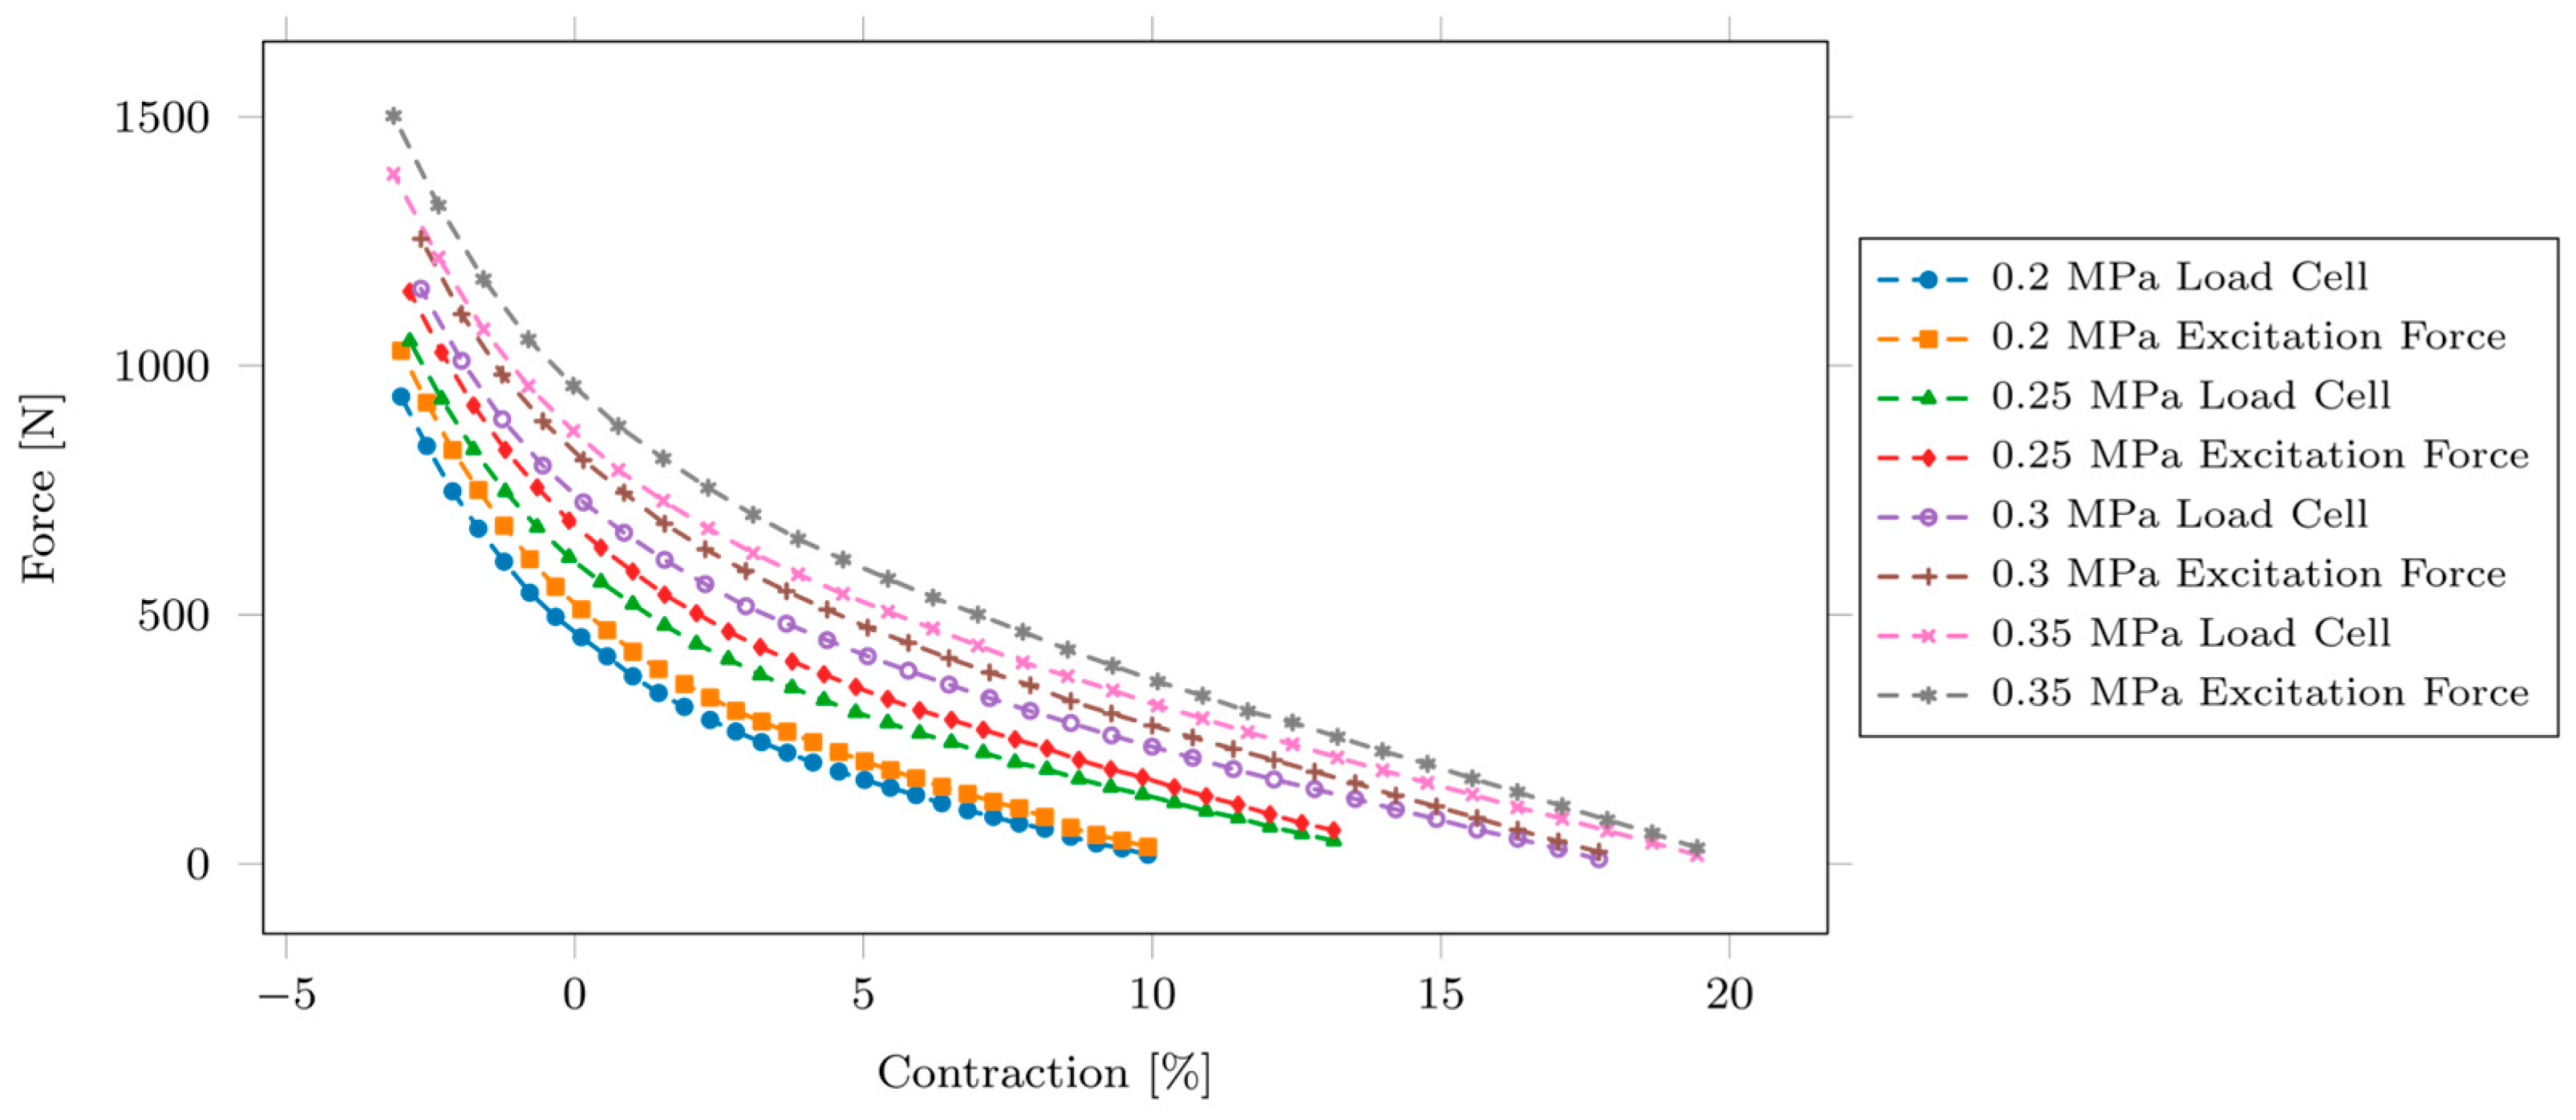
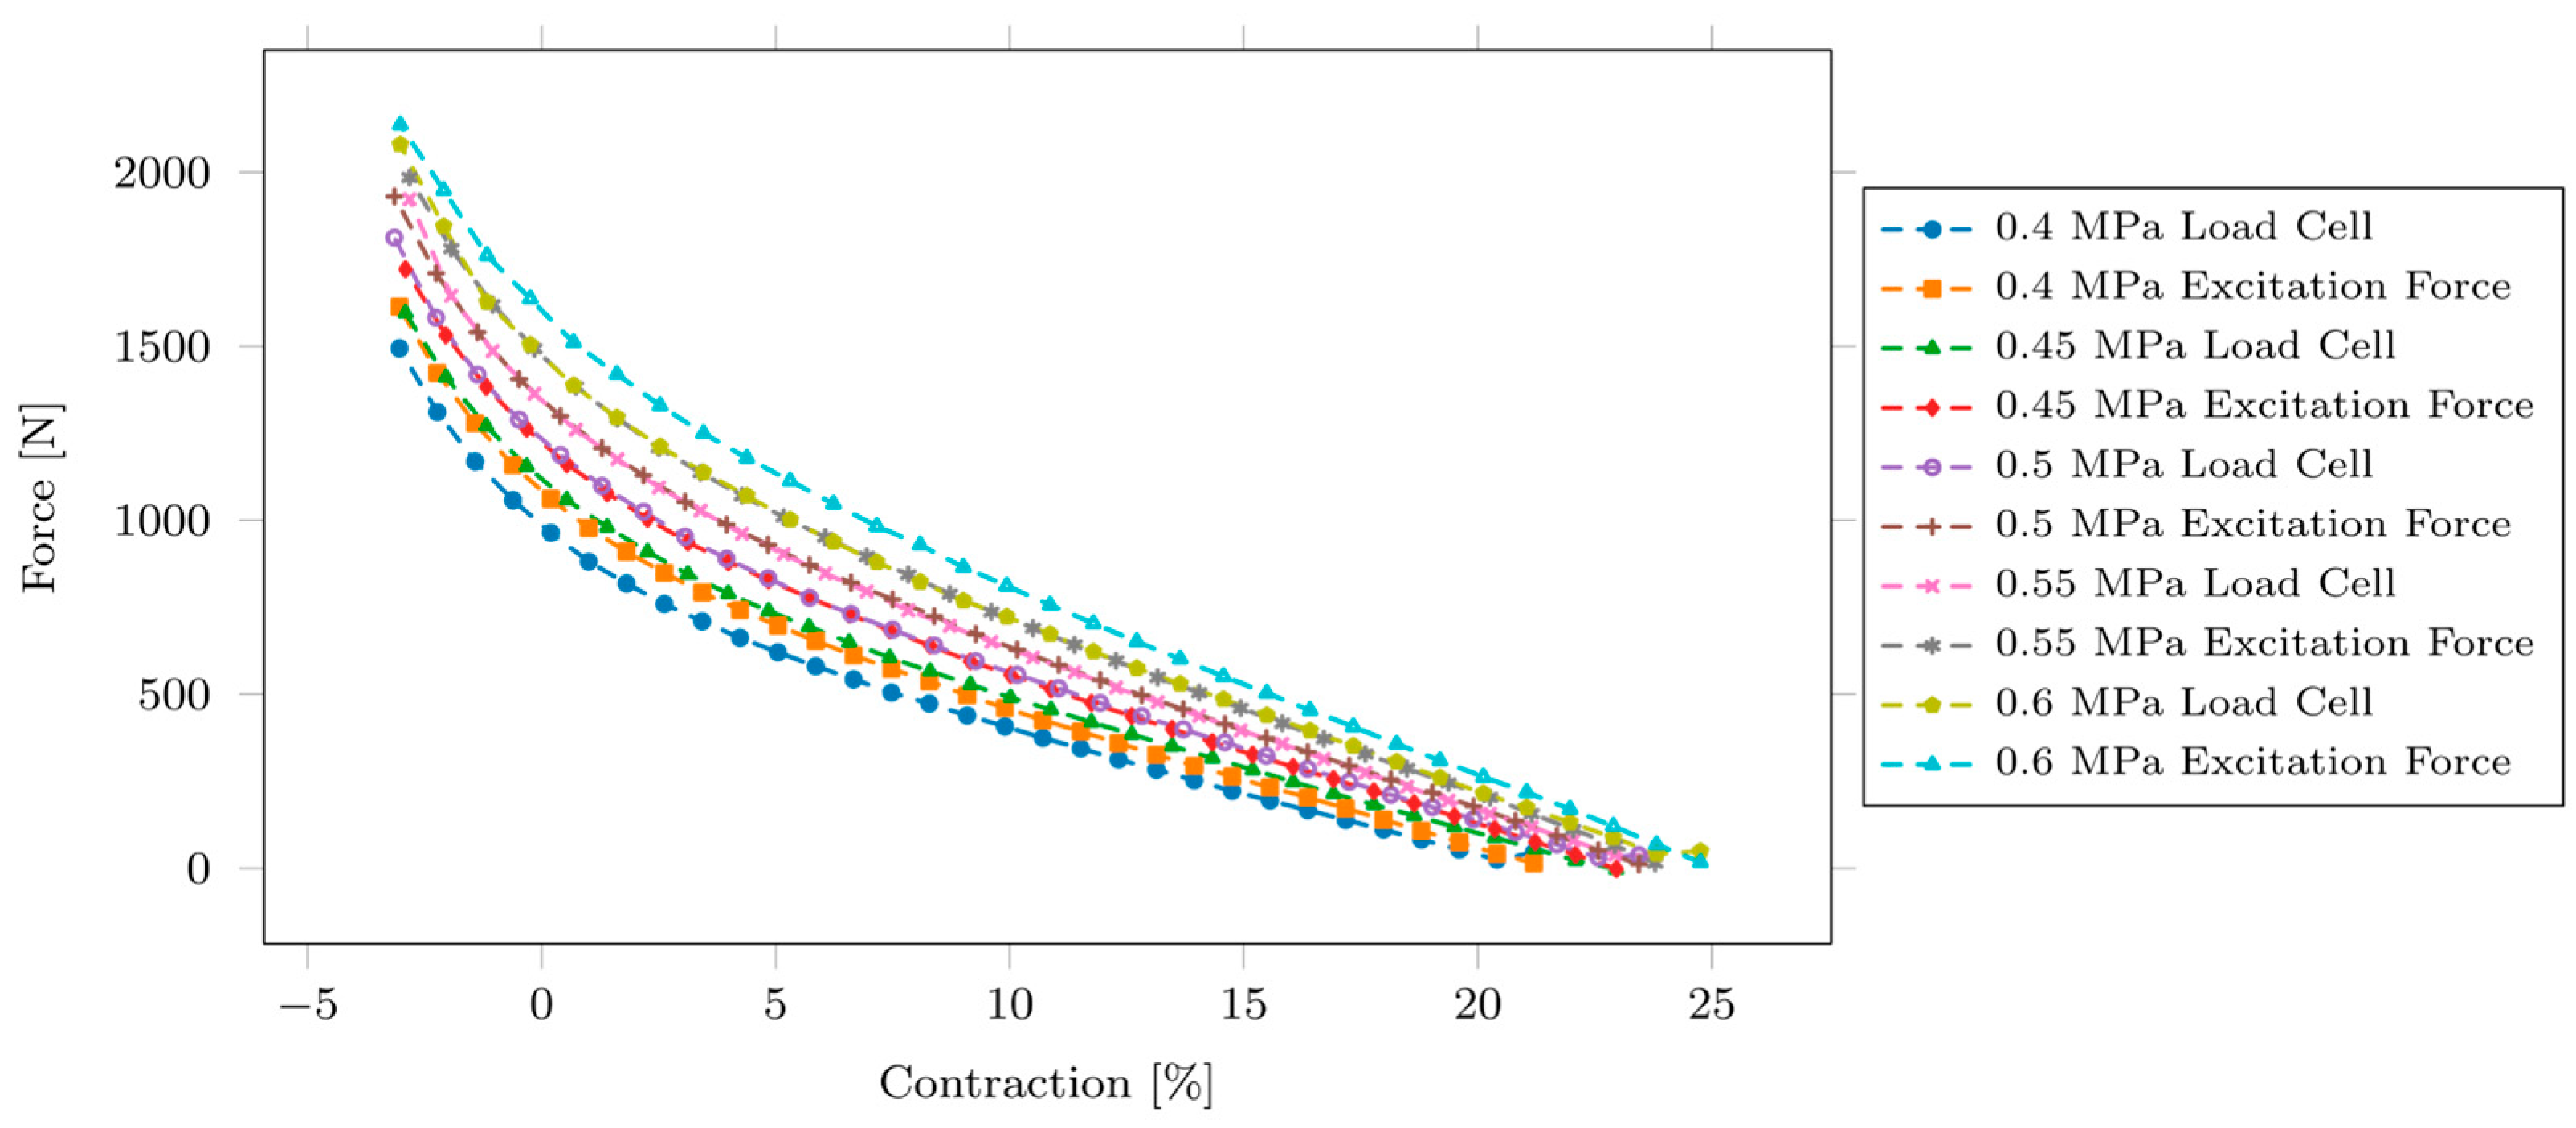
To visualize the difference between excitation and measured force on the unloading side, additional figures were created that show Fexcitation and Fmeasured as functions of contraction for both muscles, again grouped into the same three pressure ranges (0–0.15 MPa, 0.2–0.35 MPa, and 0.4–0.6 MPa) (Figure 16, Figure 17, Figure 18, Figure 19, Figure 20 and Figure 21). These expansion path plots (Figure 22, Figure 23, Figure 24, Figure 25, Figure 26 and Figure 27) highlight the larger Fexcitation–Fmeasured mismatch and the additional local loop observed in the commercial DMSP-20-200N muscle compared to the more regular single-loop behavior of the CPAM.
Figure 16.
Comparing CPAM during contraction: load cell and excitation force (0–0.15 MPa).
Figure 17.
Comparing CPAM during contraction: load cell and excitation force (0.2–0.35 MPa).
Figure 18.
Comparing CPAM during contraction: load cell and excitation force (0.4–0.6 MPa).
Figure 19.
Comparing DMSP during contraction: load cell and excitation force (0–0.15 MPa).
Figure 20.
Comparing DMSP during contraction: load cell and excitation force (0.2–0.35 MPa).
Figure 21.
Comparing DMSP during contraction: load cell and excitation force (0.4–0.6 MPa).
Figure 22.
Comparing CPAM during expansion: load cell and excitation force (0–0.15 MPa).
Figure 23.
Comparing CPAM during expansion: load cell and excitation force (0.2–0.35 MPa).
Figure 24.
Comparing CPAM during expansion: load cell and excitation force (0.4–0.6 MPa).
Figure 25.
Comparing DMSP during expansion: load cell and excitation force (0–0.15 MPa).
Figure 26.
Comparing DMSP during expansion: load cell and excitation force (0.2–0.35 MPa).
Figure 27.
Comparing DMSP during expansion: load cell and excitation force (0.4–0.6 MPa).
3.4. Hysteresis Based on Excitation Force
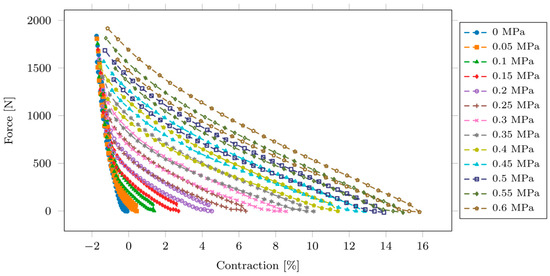
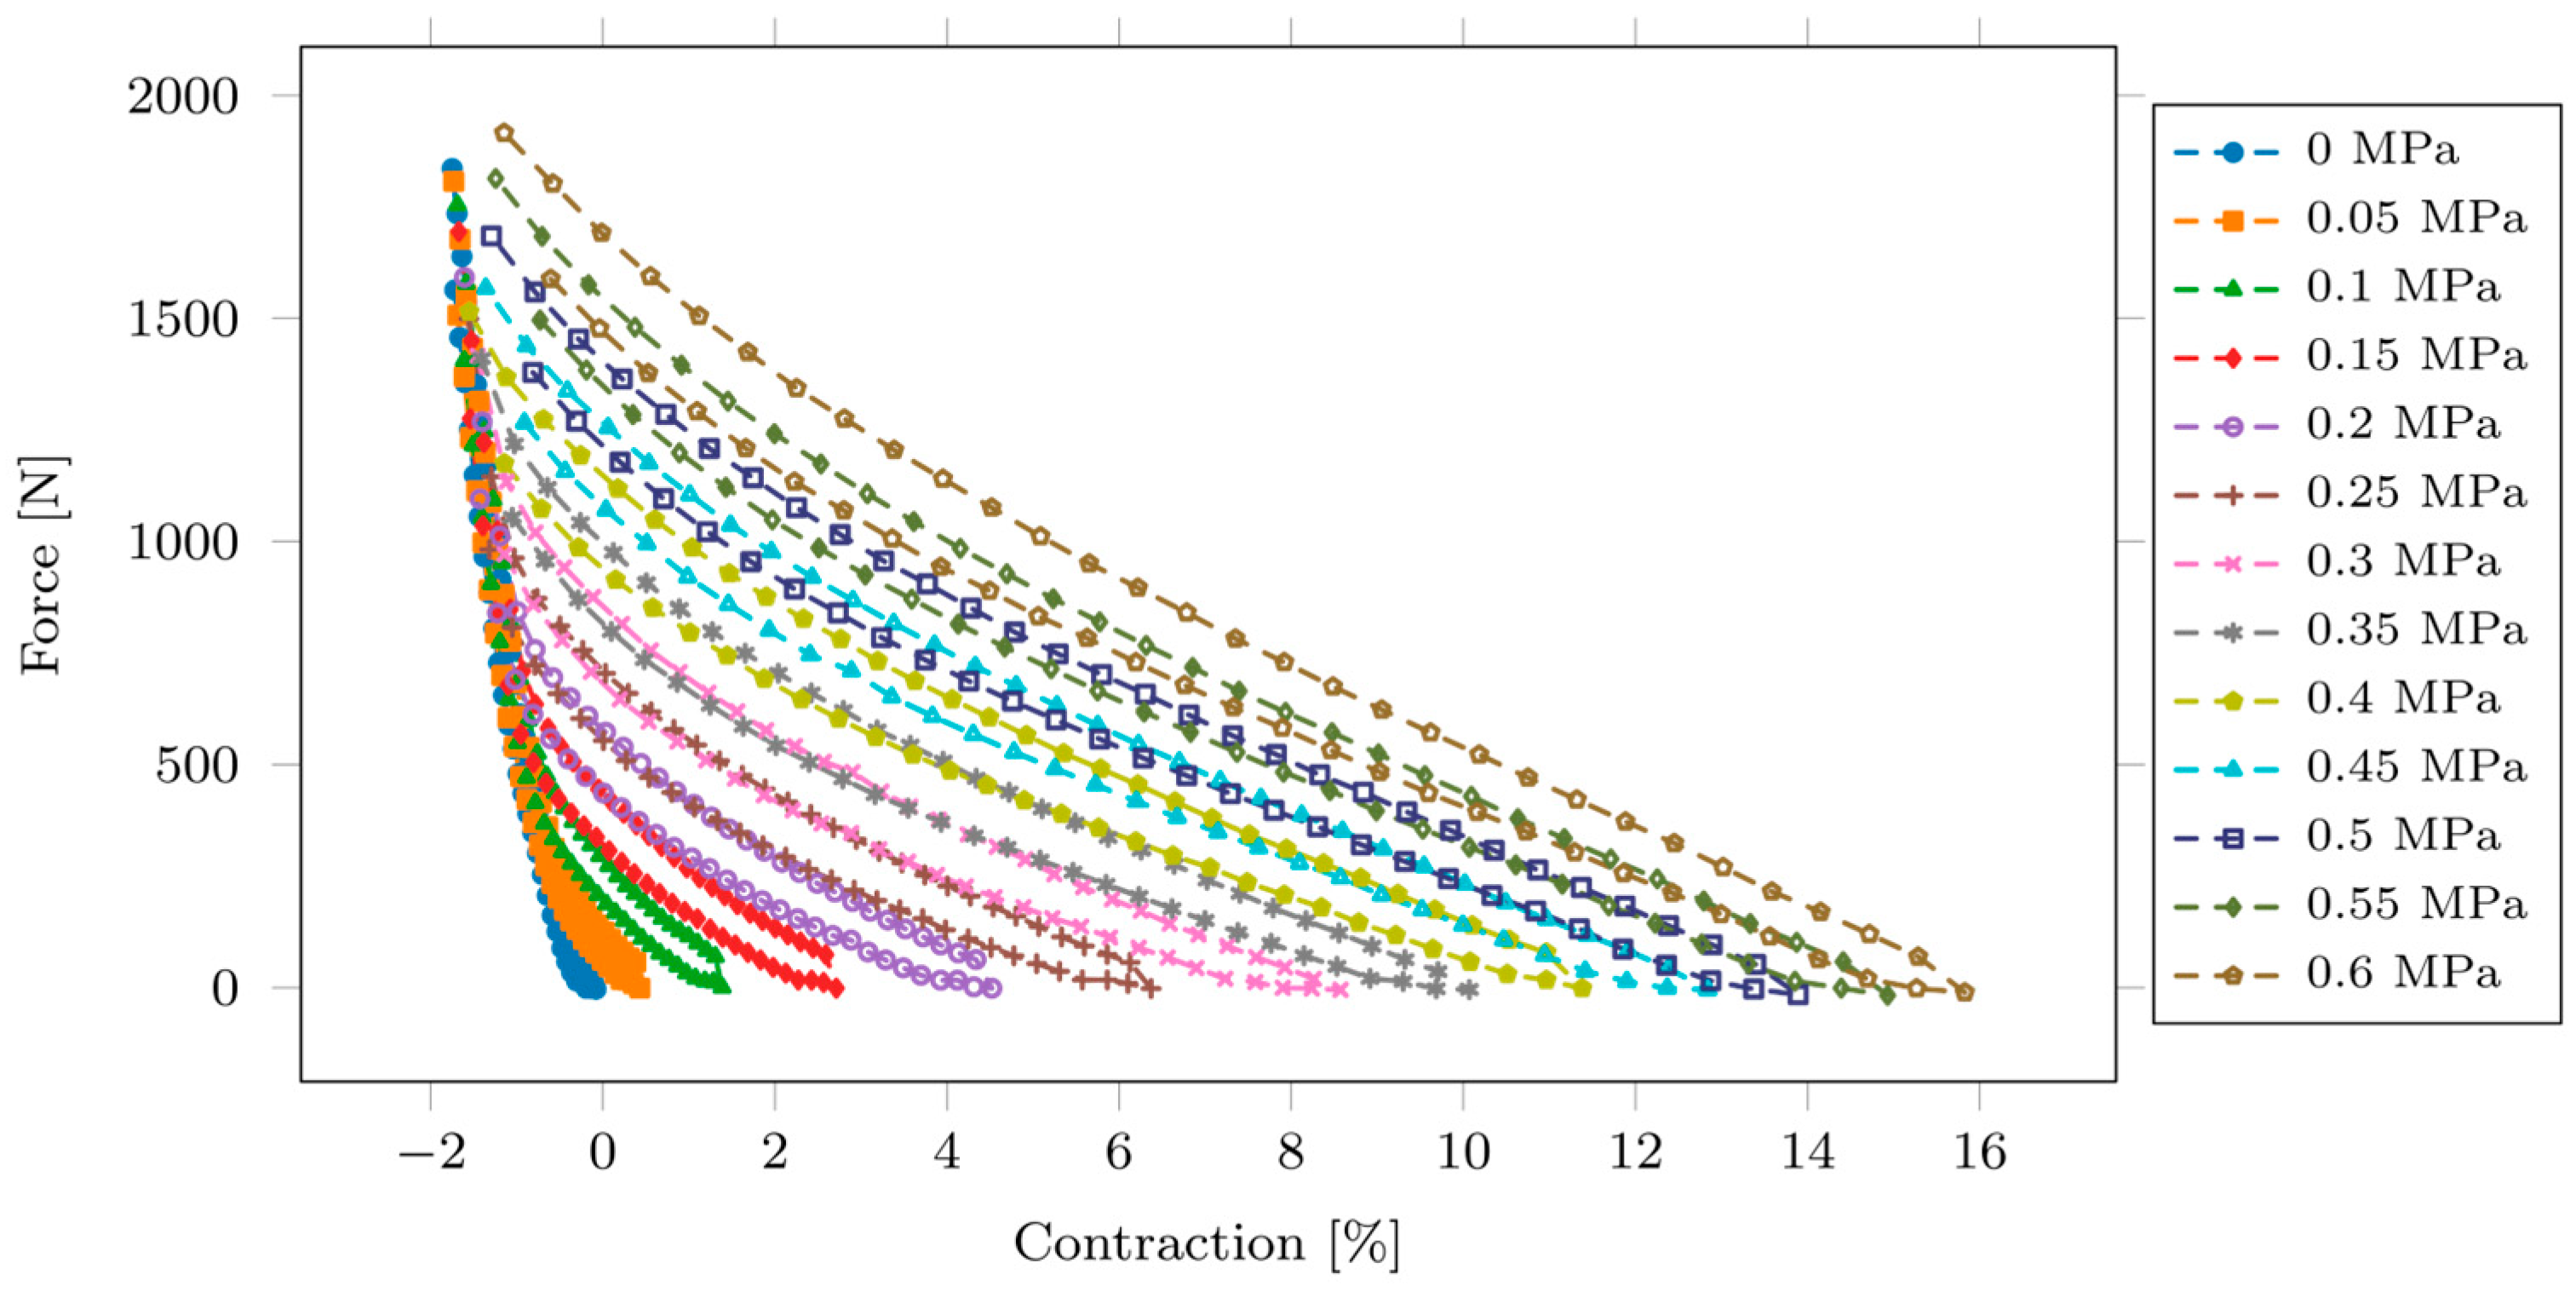
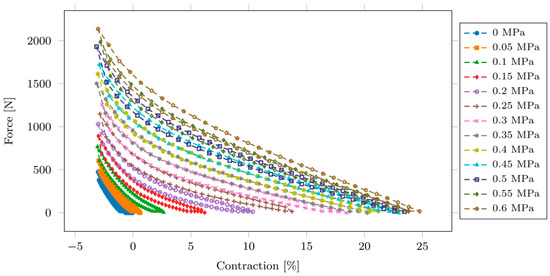
Figure 28 and Figure 29 show the hysteresis based on excitation force. To quantify hysteresis, the area enclosed by each median force–contraction loop was computed using Equation (3) for both the excitation force Fexcitation and the measured force, after which it was normalized by the maximum force and common contraction range at that pressure using Equation (4). The resulting normalized hysteresis index (HI) is summarized in Table 3, together with the indices obtained from the measured muscle force.
Figure 28.
CPAM hysteresis of excitation force.
Figure 29.
DMSP hysteresis of excitation force.
Table 3.
Calculated HI values.
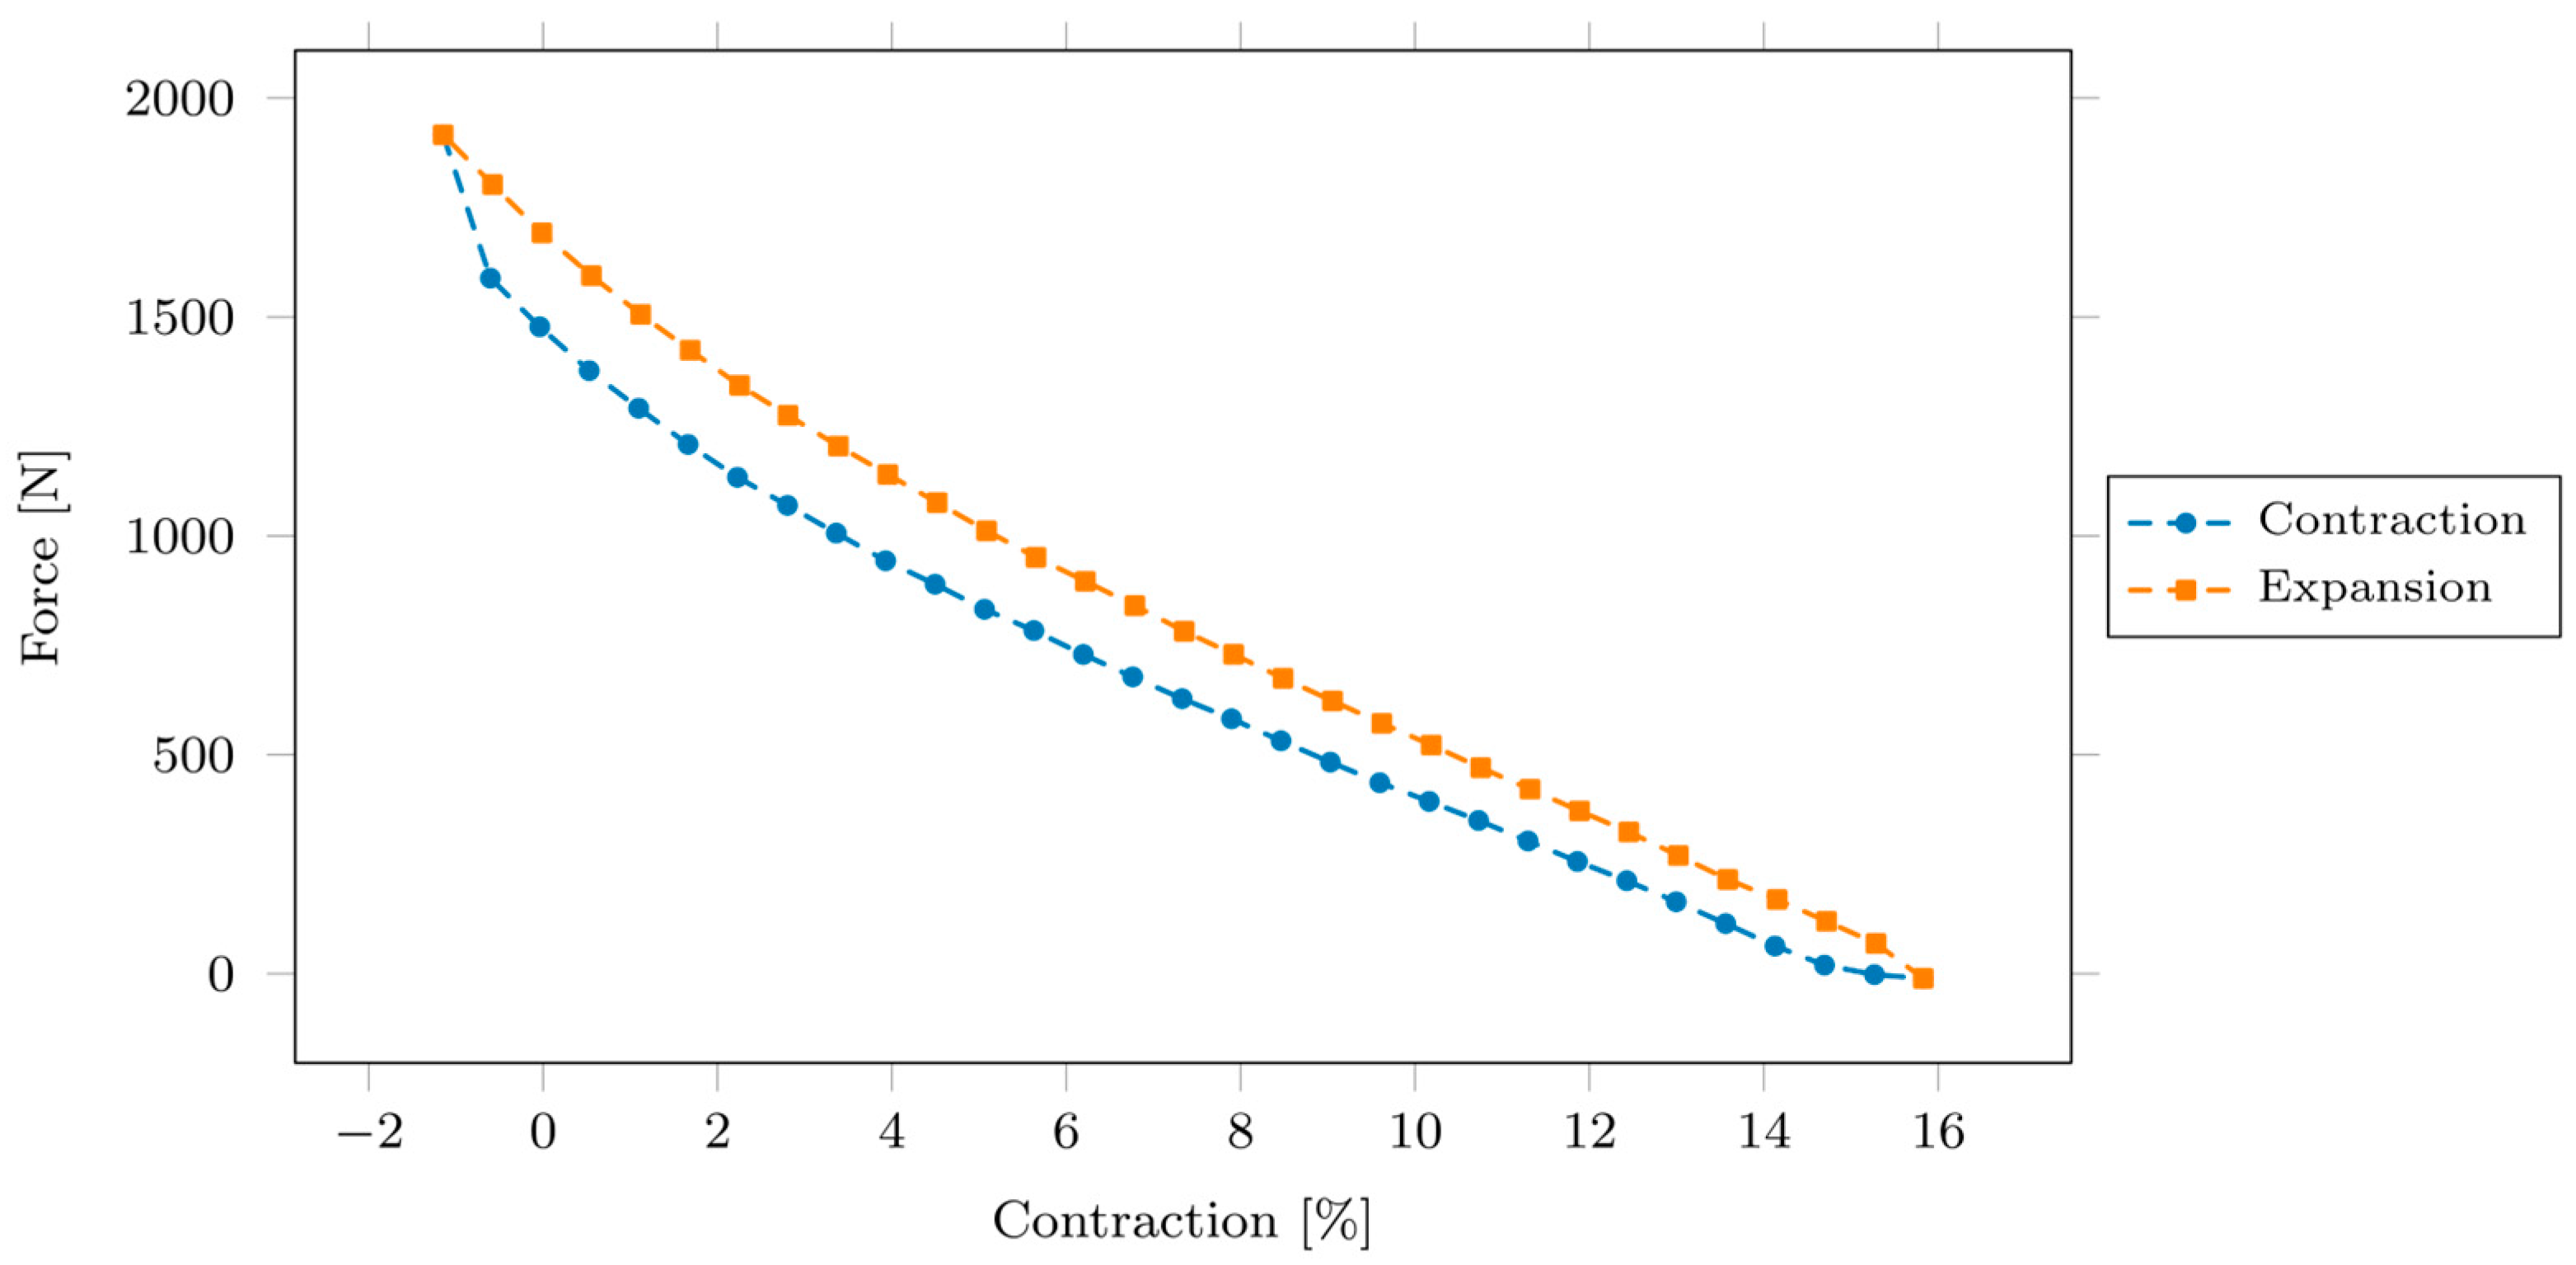
For a better visual of the loading and unloading branches of the hysteresis plot, see Figure 30, where we depict only the CPAM hysteresis of the excitation force at 0.6 MPa.
Figure 30.
Standalone image of CPAM 0.6 MPa excitation force hysteresis loop.
Where the lower branch corresponds to the contracting path and the upper branch to the expanding path. At low pressures between about 0.05 and 0.25 MPa, the CPAM exhibits a clearly lower excitation-based hysteresis index than the commercial DMSP-20-200N muscle, with reductions of 10–25% (Table 3). Around 0.30 MPa, the indices of the two muscles are remarkably similar. At higher pressures between 0.35 and 0.60 MPa, the CPAM shows a slightly larger normalized excitation-based hysteresis (about 6–12% higher). Overall, this indicates that at lower load levels, the internal spring–rod structure reduces the relative hysteresis seen from the pneumatic drive, whereas at higher pressures, additional internal deformation and friction partly offset this benefit.
3.5. Hysteresis Based on Measured Muscle Force
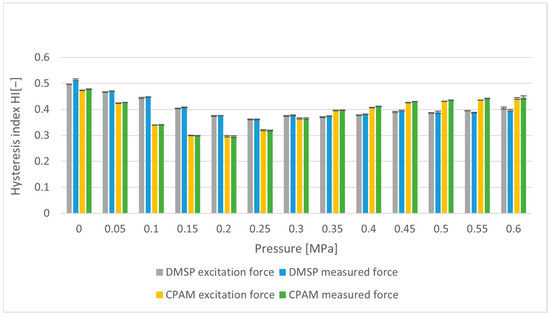
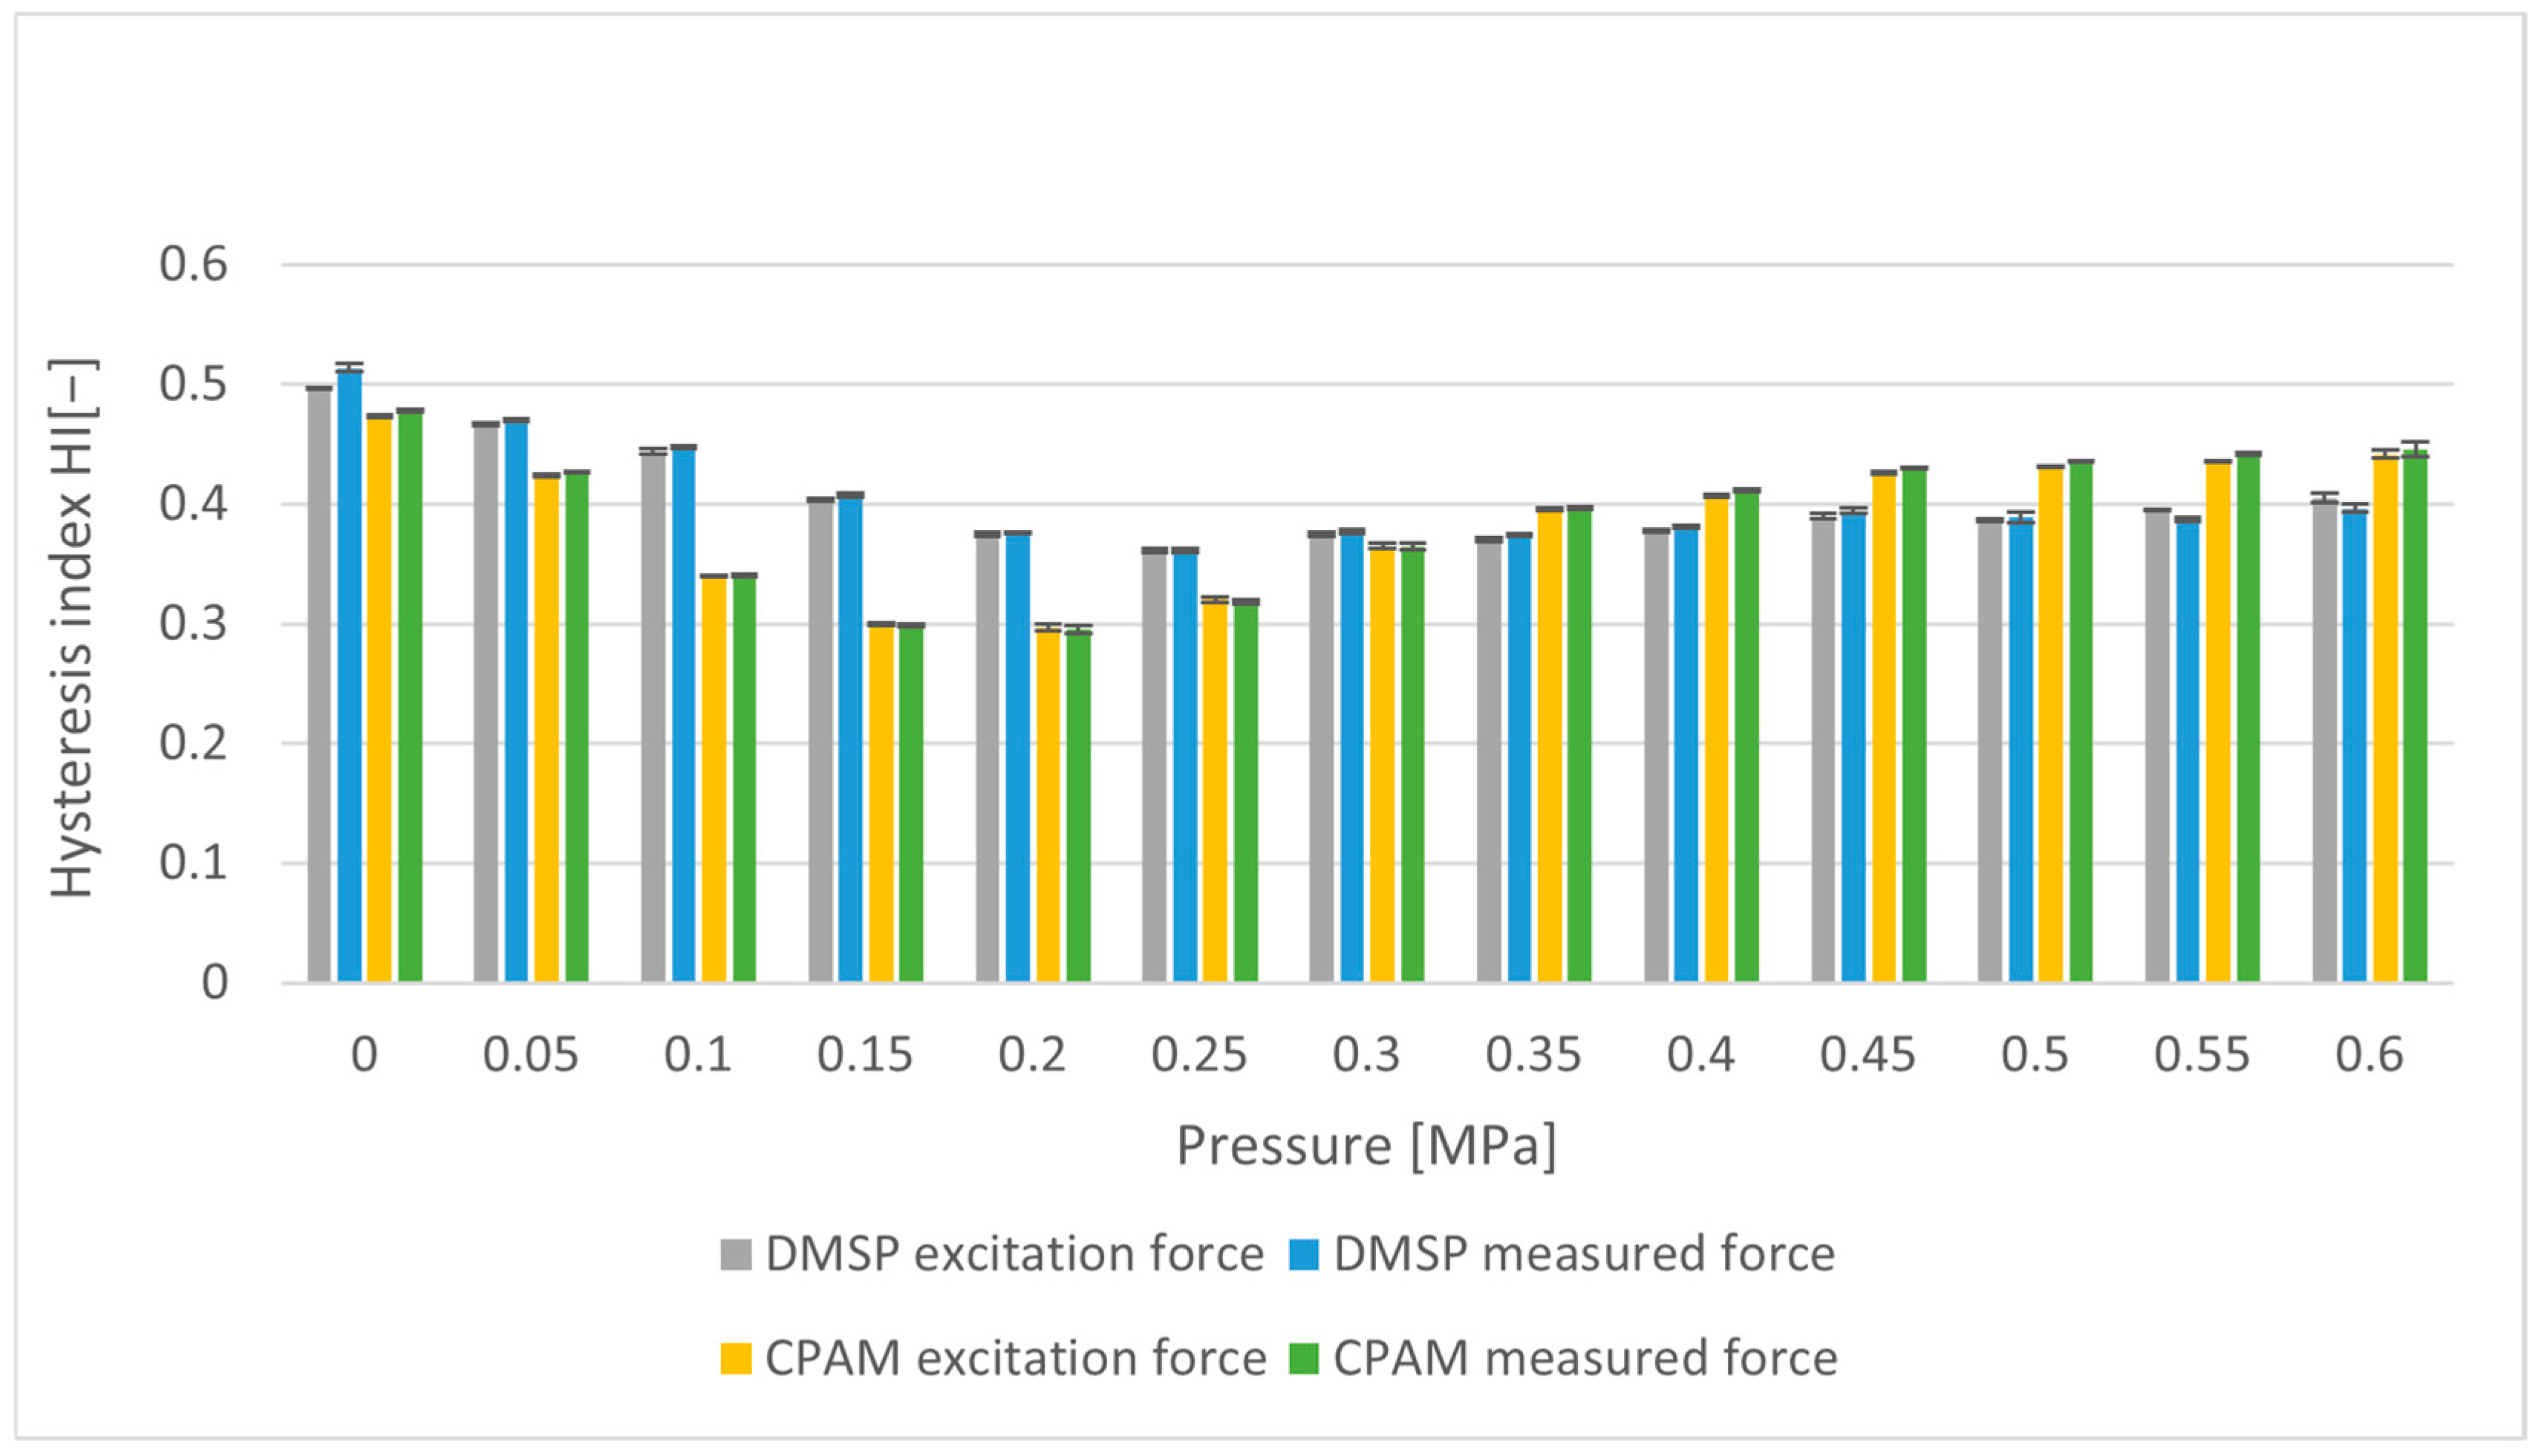
Figure 31 and Figure 32 show the hysteresis according to force measured by the load cell. A second hysteresis index was computed using the measured muscle force Fmeasured from the load cell instead of the excitation force. The same procedure was applied for each measurement: loading and unloading curves were constructed for each pressure, the loop area was integrated, and the result was normalized by the maximum measured force and the common contraction interval. Using the 5 HI values at each pressure, we performed a Student’s t distribution to calculate the confidence interval. The resulting HI(Fmeasured) numerical values are listed in Table 1 alongside the calculated CI95% values. To better visualize the results, Figure 33 presents the data in Table 3 as a bar graph.
Figure 31.
CPAM hysteresis of measured force.
Figure 32.
DMSP hysteresis of measured force.
Figure 33.
HI values across pressures.
When hysteresis is evaluated from the measured muscle force, the trends are similar to the excitation-based case. As shown in Figure 23, Figure 24, Figure 25 and Figure 26 and Table 1, the CPAM has a noticeably lower normalized hysteresis index than the DMSP-20-200N at pressures between 0.05 and 0.25 MPa (reductions of about 9–26%). Around 0.30 MPa, the indices are nearly equal, while at higher pressures, the CPAM exhibits a modestly larger normalized hysteresis (approximately 6–14% higher). This suggests that the spring–rod architecture reduces relative hysteresis in the low-pressure regime, where the additional elastic element dominates the behavior, but at higher pressures, the increased internal complexity introduces extra dissipative mechanisms so that the normalized output-side hysteresis does not decrease further and can even become slightly larger than that of the simpler commercial muscle.
3.6. Summary of Key Differences
The main experimental findings from the comparison between the commercial DMSP-20-200N muscle and the CPAM can be summarized as follows:
- Under identical rated loading conditions (2000 N at 0.6 MPa), the CPAM stretches less (about −1.5%) than the commercial muscle (about −3%), indicating a higher tensile stiffness in extension.
- During quasi-static contraction at fixed pressure, the CPAM exhibits a slightly smaller contraction range but higher force levels than the commercial muscle.
- The DMSP-20-200 muscle shows reproducible, pinched force–contraction loops with low cycle-to-cycle variability over the five repeats.
- At low pressures (approximately 0.05–0.25 MPa), the CPAM has a significantly lower normalized hysteresis index than the commercial muscle when evaluated from both the excitation force and the measured muscle force (reductions up to about 25%).
- Near 0.30 MPa, the normalized hysteresis indices of the two muscles are very similar.
- At higher pressures (0.35–0.60 MPa), the CPAM exhibits a slightly larger normalized hysteresis (roughly 6–14% higher) than the commercial muscle for both excitation-based and measured-force metrics.
These results indicate that the internal spring–rod architecture of the CPAM changes both the effective stiffness and the distribution of energy storage and dissipation in the muscle. At lower pressures, the additional elastic element reduces the relative hysteresis and makes the actuator’s behavior more spring-like. At higher pressures, however, increased internal deformation and friction in the combined spring–muscle system introduces additional dissipation so that the normalized hysteresis does not decrease further and can exceed that of the simpler commercial muscle.
4. Discussion
This work compared the quasi-static behavior of a commercial McKibben-type pneumatic artificial muscle (DMSP-20-200N) and a compact pneumatic artificial muscle (CPAM) with an internal spring–rod structure under identical boundary conditions. The two actuators share the same outer geometry and materials and were tested over the same pressure range using the same force-controlled loading protocol so that the main design difference is the presence of the internal spring and rod in the CPAM. The measurements provide insight into how this internal structure modifies stiffness, contraction behavior and hysteresis.
Prior attempts to reduce the hysteresis of PAMs rely on changing the outer muscle architecture (e.g., pleated muscles) or adding external mechanical elements (springs, linkages, frames) around the PAM. By contrast with CPAM, the load-bearing elements (rod and spring) are housed within the actuator envelope, preserving the standard McKibben bladder-braid structure and end fittings. This change in the internal structure constrains the membrane deformation, which reshapes the force–contraction loops in a pressure-dependent way. The measurements also show an important tradeoff, which is that the CPAM does not reduce the normalized hysteresis uniformity across the full pressure range. Instead, it reduces normalized hysteresis at low pressures while slightly increasing it at higher pressures. This pressure-dependent crossover is a key technical outcome of the study and should be emphasized as a design guideline rather than framed as an unconditional hysteresis reduction.
The first result is that the CPAM is noticeably stiffer in extension than the commercial muscle. Under the maximum rated load of 2000 N at 0.6 MPa specified in the DMSP-20-200N data sheet, the commercial muscle elongated by about −3% relative to its free length, whereas the CPAM elongated by only about −1.5%. This is consistent with the spring having approximately the same diameter as the rubber membrane in the stretched state, which prevents the membrane from bowing inward as in the plain McKibben architecture and forces more of the extension load into the axial spring.
Despite this higher extension stiffness, the CPAM still produces higher forces than the commercial muscle over most of the contraction range at a given pressure. The force–contraction curves show the expected monotonic trends, with similar qualitative shapes for both actuators, but the CPAM achieves slightly smaller maximum contraction and higher force levels. This behavior is compatible with a simple “spring-in-parallel” interpretation, in which the internal spring carries part of the load while the outer muscle contributes to the pressure-dependent component.
The hysteresis analysis reveals a more nuanced picture. When hysteresis is quantified through a normalized loop area based on the excitation force, the CPAM exhibits a clearly lower hysteresis index than the commercial muscle at low pressures (approximately 0.05–0.25 MPa), with reductions on the order of 10–25%. Around 0.30 MPa, the normalized indices are very similar, whereas at higher pressures (0.35–0.60 MPa), the CPAM shows a slightly larger normalized excitation-based hysteresis (about 6–12% higher). An almost identical trend is observed when hysteresis is evaluated from the measured muscle force instead of the excitation force, with low-pressure reductions up to about 25% and a modest increase at high pressures. These results suggest that the spring–rod architecture reduces relative hysteresis in the low-pressure regime, where the additional elastic element dominates the overall response, but at higher pressures, additional internal deformation and friction in the combined spring–muscle system introduce extra dissipation so that the normalized hysteresis no longer decreases and can even become slightly larger than that of the simpler commercial muscle.
The detailed loop shapes during unloading further support this interpretation. The commercial DMSP-20-200N often exhibits a small additional loop or kink on the expansion side, together with a larger mismatch between the excitation force and the measured muscle force. This indicates that a non-negligible fraction of the work delivered by the cylinder is dissipated or stored internally in the commercial muscle without being transmitted to the load. In contrast, the CPAM shows a more regular single-loop behavior and a smaller excitation–measured force difference on the expansion side, consistent with a more constrained internal deformation pattern imposed by the spring and rod.
From the perspective of mechanical mem-elements, both actuators display force–contraction loops characteristic of history-dependent behavior, but the CPAM shifts the balance between elastic and hysteretic contributions. At lower pressures, its behavior is closer to that of an ideal elastic element with a modest hysteresis correction, which may simplify modeling and control and could be advantageous for implementations that use PAMs as mechanical analogs of memristive elements. At higher pressures, however, the added internal structure does not eliminate hysteresis and instead redistributes dissipative mechanisms, so that the overall normalized hysteresis is not reduced across the entire operating range.
Many PAM-driven systems in soft robotics and rehabilitation operate in the low to moderate pressure range to preserve compliance and safety. In this range (0.05–0.25 MPa), the 10–25% reduction in normalized hysteresis implies a smaller effective deadband between the loading and unloading curves and less history-dependent error for the control model or feedforward positioning. This can reduce calibration effort for open-loop systems. The CPAM architecture can also simplify mechanical integration since the spring and rod are internal and do not require external linkages or antagonistic mechanisms.
Since the inside of the muscle is filled with the rod and spring, the effective pneumatic volume is reduced compared to a hollow McKibben muscle, which should reduce pneumatic capacitance and thereby increase pressure response for a given mass-flow capability. Future work should quantify this expected responsiveness benefit directly.
Several limitations should be noted. First, only one specimen of each muscle type was tested, so manufacturing variability and aging effects were not assessed. Second, the experiments were restricted to quasi-static loading at a single force rate of approximately 4 N/s; dynamic behavior and rate-dependent hysteresis were not explored. Third, temperature effects and long-term drift were not systematically measured, and the internal pressure distribution and local braid deformation inside the CPAM remain unobserved. Finally, the normalization of hysteresis by peak force and common contraction range facilitates comparison between muscles and pressures, but other normalization choices could emphasize different aspects of the behavior.
Future work could address these limitations by testing multiple specimens, extending the measurements to dynamic regimes and cyclic fatigue, and combining the macroscopic force–contraction data with local strain or temperature measurements on the muscle surface. It would also be useful to develop compact phenomenological models that capture the pressure-dependent transition from reduced to increased normalized hysteresis in the CPAM and to explore how such actuators behave in closed-loop control and in mechanical computing or memory architectures.
5. Conclusions
This study introduced and experimentally characterized a compact pneumatic artificial muscle (CPAM) that integrates an internal spring and rod into a McKibben-type outer muscle and compared its behavior to a commercial DMSP-20-200N actuator under identical loading conditions. By matching outer geometry, materials, and operating pressures, the influence of the internal spring–rod architecture on stiffness and hysteresis could be isolated.
The results show that the CPAM is stiffer in extension and produces higher forces over most of the contraction range than the commercial muscle, while achieving a slightly smaller maximum contraction. When hysteresis is quantified via the normalized loop area, the CPAM exhibits substantially lower normalized hysteresis than the DMSP-20-200N at low pressures, similar hysteresis at intermediate pressures, and a modestly higher normalized hysteresis at the upper end of the pressure range. The detailed unloading loops and the comparison between excitation and measured forces indicate that the spring–rod structure constrains internal deformation and reduces relative hysteresis in the low-pressure regime but also introduces additional dissipative mechanisms at higher pressures.
Overall, the CPAM shifts the balance between elastic and hysteretic behavior in a way that makes the actuator more spring-like at lower pressures, which may simplify modeling and control and is promising for applications that exploit PAMs as mechanical analogs of memristive elements. At the same time, the persistence and partial re-emergence of hysteresis at higher pressures highlight that internal structural modifications do not eliminate hysteresis but reshape how and where energy is stored and dissipated. The methodology developed here—side-by-side comparison under matched conditions, normalization of hysteresis by peak force and contraction range, and separate evaluation of excitation and output forces—provides a basis for systematically assessing future PAM designs with tailored internal structures.
Author Contributions
Conceptualization, S.C.; methodology, S.C.; software, S.C.; validation, S.C.; formal analysis, S.C.; investigation, S.C.; resources, J.S.; data curation, S.C.; writing—original draft preparation, S.C.; writing—review and editing, S.C. and A.M.; visualization, S.C.; supervision, J.S.; project administration, A.M.; funding acquisition, J.S. All authors have read and agreed to the published version of the manuscript.
Funding
This research received no external funding.
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
Dataset available on request from the authors.
Conflicts of Interest
The authors declare no conflict of interest.
References
- Daerden, F.; Lefeber, D. Pneumatic artificial muscles: Actuators for robotics and automation. Eur. J. Mech. Environ. Eng. 2002, 47, 11–21. [Google Scholar]
- Tondu, B. Modelling of the McKibben artificial muscle: A review. J. Intell. Mater. Syst. Struct. 2012, 23, 225–253. [Google Scholar] [CrossRef] [Scilit]
- Al-Mayahi, W.; Al-Fahaam, H. A Review of Design and Modeling of Pneumatic Artificial Muscle. IJEEE 2024, 20, 122–136. [Google Scholar] [CrossRef] [Scilit]
- Andrikopoulos, G.; Nikolakopoulos, G.; Manesis, S. A Survey on applications of Pneumatic Artificial Muscles. In Proceedings of the 2011 19th Mediterranean Conference on Control & Automation (MED), Corfu, Greece, 20–23 June 2011; IEEE: Corfu, Greece, 2011; pp. 1439–1446. [Google Scholar]
- Al-Fahaam, H.; Davis, S.; Nefti-Meziani, S. The design and mathematical modelling of novel extensor bending pneumatic artificial muscles (EBPAMs) for soft exoskeletons. Robot. Auton. Syst. 2018, 99, 63–74. [Google Scholar] [CrossRef] [Scilit]
- Kalita, B.; Dwivedy, S.K. Dynamic analysis of pneumatic artificial muscle (PAM) actuator for rehabilitation with principal parametric resonance condition. Nonlinear Dyn 2019, 97, 2271–2289. [Google Scholar] [CrossRef] [Scilit]
- Chou, C.-P.; Hannaford, B. Measurement and modeling of McKibben pneumatic artificial muscles. IEEE Trans. Robot. Automat. 1996, 12, 90–102. [Google Scholar] [CrossRef] [Scilit]
- Tondu, B.; Lopez, P. Modeling and control of McKibben artificial muscle robot actuators. IEEE Control Syst. 2000, 20, 15–38. [Google Scholar] [CrossRef] [Scilit]
- Tsagarakis, N.; Caldwell, D.G. Improved modelling and assessment of pneumatic muscle actuators. In Proceedings of the 2000 ICRA. Millennium Conference. IEEE International Conference on Robotics and Automation. Symposia Proceedings (Cat. No.00CH37065), San Francisco, CA, USA, 24–28 April 2000; IEEE: San Francisco, CA, USA, 2000; Volume 4, pp. 3641–3646. [Google Scholar]
- Klute, G.K.; Hannaford, B. Accounting for Elastic Energy Storage in McKibben Artificial Muscle Actuators. J. Dyn. Syst. Meas. Control. 2000, 122, 386–388. [Google Scholar] [CrossRef] [Scilit]
- Kothera, C.S.; Jangid, M.; Sirohi, J.; Wereley, N.M. Experimental Characterization and Static Modeling of McKibben Actuators. J. Mech. Des. 2009, 131, 091010. [Google Scholar] [CrossRef] [Scilit]
- Wickramatunge, K.C.; Leephakpreeda, T. Study on mechanical behaviors of pneumatic artificial muscle. Int. J. Eng. Sci. 2010, 48, 188–198. [Google Scholar] [CrossRef] [Scilit]
- Davis, S.; Caldwell, D.G. Braid Effects on Contractile Range and Friction Modeling in Pneumatic Muscle Actuators. Int. J. Robot. Res. 2006, 25, 359–369. [Google Scholar] [CrossRef] [Scilit]
- Andrikopoulos, G.; Nikolakopoulos, G.; Manesis, S. Incorporation of thermal expansion in static force modeling of Pneumatic Artificial Muscles. In Proceedings of the 2015 23rd Mediterranean Conference on Control and Automation (MED), Torremolinos, Spain, 16–19 June 2015; IEEE: Malaga, Spain, 2015; pp. 414–420. [Google Scholar]
- Wang, G.; Hua, X.; Xu, J.; Song, L.; Chen, K. Analysis, modeling and experimental validation of temperature-changing effect on mechanical properties of pneumatic artificial muscle. Adv. Robot. 2018, 32, 984–998. [Google Scholar] [CrossRef] [Scilit]
- Kadowaki, J.; Sasaki, D.; Yase, H.; Kimura, T. Modeling the hysteresis characteristics of McKibben type artificial rubber muscle based on rubber physical characteristics. Trans. JSME 2022, 88, 21–00290-21–00290. [Google Scholar] [CrossRef] [Scilit]
- Cveticanin, L.; Zukovic, M.; Biro, I.; Sarosi, J. Mathematical investigation of the stability condition and steady state position of a pneumatic artificial muscle—Mass system. Mech. Mach. Theory 2018, 125, 196–206. [Google Scholar] [CrossRef] [Scilit]
- Vo-Minh, T.; Tjahjowidodo, T.; Ramon, H.; Van Brussel, H. A New Approach to Modeling Hysteresis in a Pneumatic Artificial Muscle Using the Maxwell-Slip Model. IEEE/ASME Trans. Mechatron. 2011, 16, 177–186. [Google Scholar] [CrossRef] [Scilit]
- Liu, Y.; Zang, X.; Lin, Z.; Liu, X.; Zhao, J. Modelling Length/Pressure Hysteresis of a Pneumatic Artificial Muscle using a Modified Prandtl-Ishlinskii Model. SV-JME 2017, 63, 56–64. [Google Scholar] [CrossRef] [Scilit]
- Al Ma Aita, M.; Al, M.; Zgoul, M. Hysteresis Nonlinearities in Pneumatic artificial Muscles. In Proceedings of the Fourth International Conference on Advances in Mechanical and Robotics Engineering—AMRE 2016, Rome, Italy, 16 December 2016; Institute of Research Engineers and Doctors: New York, NY, USA, 2016; pp. 6–10. [Google Scholar]
- Nguyen, M.K.; Trinh, V.C.; Vo, N.Y.P.; Le, T.D. Restoring Model of a Pneumatic Artificial Muscle with Structure Parameters: Analysis and Identification. Actuators 2024, 13, 355. [Google Scholar] [CrossRef] [Scilit]
- Sokolov, O.; Csikos, S.; Hosovsky, A.; Sarosi, J.; Sokolov, S. Hysteresis Compensation of Pneumatic Artificial Muscles Using Correctional Curve Offset: Case Study. In Advances in Design, Simulation and Manufacturing VII; Ivanov, V., Pavlenko, I., Edl, M., Machado, J., Xu, J., Eds.; Lecture Notes in Mechanical Engineering; Springer Nature: Cham, Switzerland, 2024; pp. 107–118. ISBN 978-3-031-63719-3. [Google Scholar]
- Daerden, F.; Lefeber, D. The Concept and Design of Pleated Pneumatic Artificial Muscles. Int. J. Fluid Power 2001, 2, 41–50. [Google Scholar] [CrossRef] [Scilit]
- Saito, N.; Satoh, T.; Saga, N. Double Air Chambers Pneumatic Artificial Muscle and Non-Hysteresis Position Control. Actuators 2024, 13, 282. [Google Scholar] [CrossRef] [Scilit]
- Sarosi, J.; Biro, I.; Nemeth, J.; Cveticanin, L. Dynamic modeling of a pneumatic muscle actuator with two-direction motion. Mech. Mach. Theory 2015, 85, 25–34. [Google Scholar] [CrossRef] [Scilit]
- Han, K.; Kim, N.-H.; Shin, D. A Novel Soft Pneumatic Artificial Muscle with High-Contraction Ratio. Soft Robot. 2018, 5, 554–566. [Google Scholar] [CrossRef] [Scilit]
- Do Rosario Carvalho, A.D.; Karanth, P.N.; Desai, V. Design and characterization of a pneumatic muscle actuator with novel end-fittings for medical assistive applications. Sens. Actuators A Phys. 2021, 331, 112877. [Google Scholar] [CrossRef] [Scilit]
- Soleymani, R.; Khajehsaeid, H. A mechanical model for McKibben pneumatic artificial muscles based on limiting chain extensibility and 3D application of the network alteration theories. Int. J. Solids Struct. 2020, 202, 620–630. [Google Scholar] [CrossRef] [Scilit]
- Liu, W.; Rahn, C.R. Fiber-Reinforced Membrane Models of McKibben Actuators. J. Appl. Mech. 2003, 70, 853–859. [Google Scholar] [CrossRef] [Scilit]
- Ball, E.; Garcia, E. Effects of Bladder Geometry in Pneumatic Artificial Muscles. J. Med. Devices 2016, 10, 041001. [Google Scholar] [CrossRef] [Scilit]
- Hocking, E.G.; Wereley, N.M. Analysis of nonlinear elastic behavior in miniature pneumatic artificial muscles. Smart Mater. Struct. 2013, 22, 014016. [Google Scholar] [CrossRef] [Scilit]
- Čakurda, T.; Trojanová, M.; Hošovský, A.; Sokolov, O. Improving the Performance of Grey-Box Model of 3-DOF Compliant Robotic Arm with Fluidic Muscles. In EAI International Conference on Automation and Control in Theory and Practice; Balog, M., Iakovets, A., Hrehova, S., Eds.; EAI/Springer Innovations in Communication and Computing; Springer Nature: Cham, Switzerland, 2023; pp. 315–334. ISBN 978-3-031-31966-2. [Google Scholar]
- FESTO DMSP Catalogue. Available online: https://www.festo.com/media/catalog/204251_documentation.pdf (accessed on 14 December 2025).

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.