


Abstract
Rodents, as a core component of desert ecosystems and an important indicator of environmental changes, are ideal subjects for studying the impacts of fluctuations in climatic conditions on wildlife. Based on field data from the southern Alxa Desert (2014–2020), this study constructed an ecosystem structure network integrating local/metacommunities, climate, soil, and plant communities. Combined with structural equation modeling, we explored the response mechanisms of rodent communities to climatic conditions across multiple scales. The results showed the following: the α-diversity of local and metacommunities exhibited convergent seasonal patterns, with greater impacts from human disturbances than interannual effects, as well as coexisting species turnover and nesting in metacommunities. Precipitation directly affected metacommunity abundance and diversity and indirectly influenced both community types via vegetation, while temperature directly regulated community characteristics; metacommunities were formed via the coupling of local communities through species migration and habitat filtering, reflecting complex links between local and regional processes. This research provides scientific support for predicting desert ecosystem dynamics and guiding conservation management.
1. Introduction
Small mammals are important indicators of habitat stability, biodiversity, and environmental change caused by human activity [1]. Rodent populations respond to environmental changes, disturbances, and habitat structural changes (succession or fragmentation) [2]. Thus, their presence and absence, population density changes, community diversity, and physical conditions can all serve as practical tools for evaluating ecosystem health [3]. The concept of “metacommunity” emerged when ecologists explored the coexistence mechanisms, diversity, local-scale properties, and processes of community species in fragmented habitats within a broader spatiotemporal framework [4]. It defines set of local communities connected by dispersal among multiple potentially interacting species [5,6]. A metacommunity’s ecosystem function, species community composition, and biodiversity are determined by considering different spatial scales and temporal dynamics, energy, resources (abiotic, biotic), traits of mammals (dispersal, life cycle, migration, and movement), and environmental conditions both between and within different spatial units [7]. The fundamental issue in metacommunity research is the mechanism of multispecies coexistence, as well as the causes and maintenance mechanisms of diversity. In some wild ecosystems, habitat fragmentation caused by climate change and other factors determines the characteristics of rodent communities in habitats through down/up-regulation [8]. Patchy habitats formed by human disturbance and climate change have become permanent. The limited diffusion of rodents between patches has endowed the rodents in the Alxa Desert with the basic characteristics of metapopulations and metacommunities [9,10]. Metacommunity theory is rapidly developing with the expansion of theoretical research, yet few experimental studies have been conducted [6,11]. Although the concept of metacommunity provides a clear explanation for the spatial dynamics and relationships of communities, there is relatively little research on its importance on a temporal scale. Therefore, integrating temporal scales into metacommunity research represents an important direction for the future development of metacommunity ecology [11]. Empirical cases of metacommunity structure research are mostly conducted within a relatively short time frame, such as studies on plankton. However, there are fewer long-term studies on metacommunities of small mammals [6,9].
Climate change over the past few decades has had a significant impact on species distribution and richness [12,13]. International research on animal responses to climate change has been extensively conducted. These studies indicate that climate change affects animal geographical distribution, phenology, individual behavior, and population dynamics. However, most studies have been conducted at larger (macro) and continental scales [14,15], and simulations have been used to predict animal responses in the coming decades [16,17]. There is relatively little research on the impact of climate change on animals at smaller scales [18]. Determining the causes of vegetation changes in arid and semiarid environments under climate change is difficult, as the factors causing vegetation changes include disturbances, soil properties, effects from past years, and the interrelationships between these factors. In these systems, models describing vegetation changes generally focus on using a single factor as the initial driver. Integrating these factors into a single model may be more conducive to fully understanding the driving mechanisms of vegetation changes in desert systems [19]. Similarly, the impact of climate change on rodents may involve multiple factors or pathways, making it necessary to integrate these factors into a single model for analysis.
One of the core scientific issues in community ecology research is biodiversity. While the potential of biodiversity to buffer ecosystems against the impacts of extreme climate change remains unconfirmed, the global prevalence of climate change-induced shifts in biodiversity has risen markedly in recent years [20]. The composition and diversity of rodent communities are significantly correlated with their habitat conditions [21,22]. Multiple factors, including climatic conditions, topography, soil physicochemical conditions, human disturbances, and scales, collectively explain the variations in the composition, diversity, and dynamic characteristics of rodent communities. The synergistic effect between land use and climate change is expected to have a more profound negative impact on biodiversity than either driving factor alone or their additive combination [23,24].
Anthropogenic disturbances (e.g., grazing and farming) have caused long-term, stable changes in natural environments. Habitat fragmentation also generates local communities, providing a basis for investigating the response mechanisms of rodent communities to climate factor changes and anthropogenic disturbances at both the local community scale (rodent communities within habitat patches) and the metacommunity scale (a collection of all local communities in the study area). We hypothesize that water and heat are the two primary limiting factors constraining desert ecosystems. In the study area, variations in temperature and precipitation, as well as the pulsed effects of extreme climatic events triggered by fluctuations in climatic conditions, may have exerted profound impacts on the desert rodents community. Local communities may be more sensitive to changes in climatic factors than metacommunities, and the response mechanisms of metacommunities to climatic conditions differ from those of local communities. This study aims to test these hypotheses, which are associated with the four paradigms of metacommunities but focus more on revealing the intrinsic mechanisms underlying the integration of local communities into the metacommunity. Scientifically, the findings of this research will enrich the theory of rodent metacommunities during habitat fragmentation. Practically, they will provide a scientific basis for formulating strategies for the restoration and protection of desert ecosystems, promoting the sustainable utilization of grassland animal husbandry, and supporting the prediction and comprehensive management of regional rodent pests.
2. Materials and Methods
2.1. Study Area
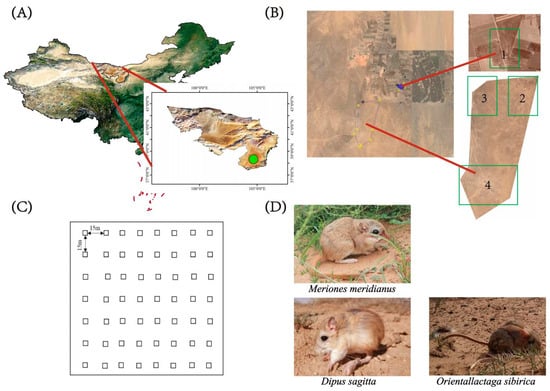
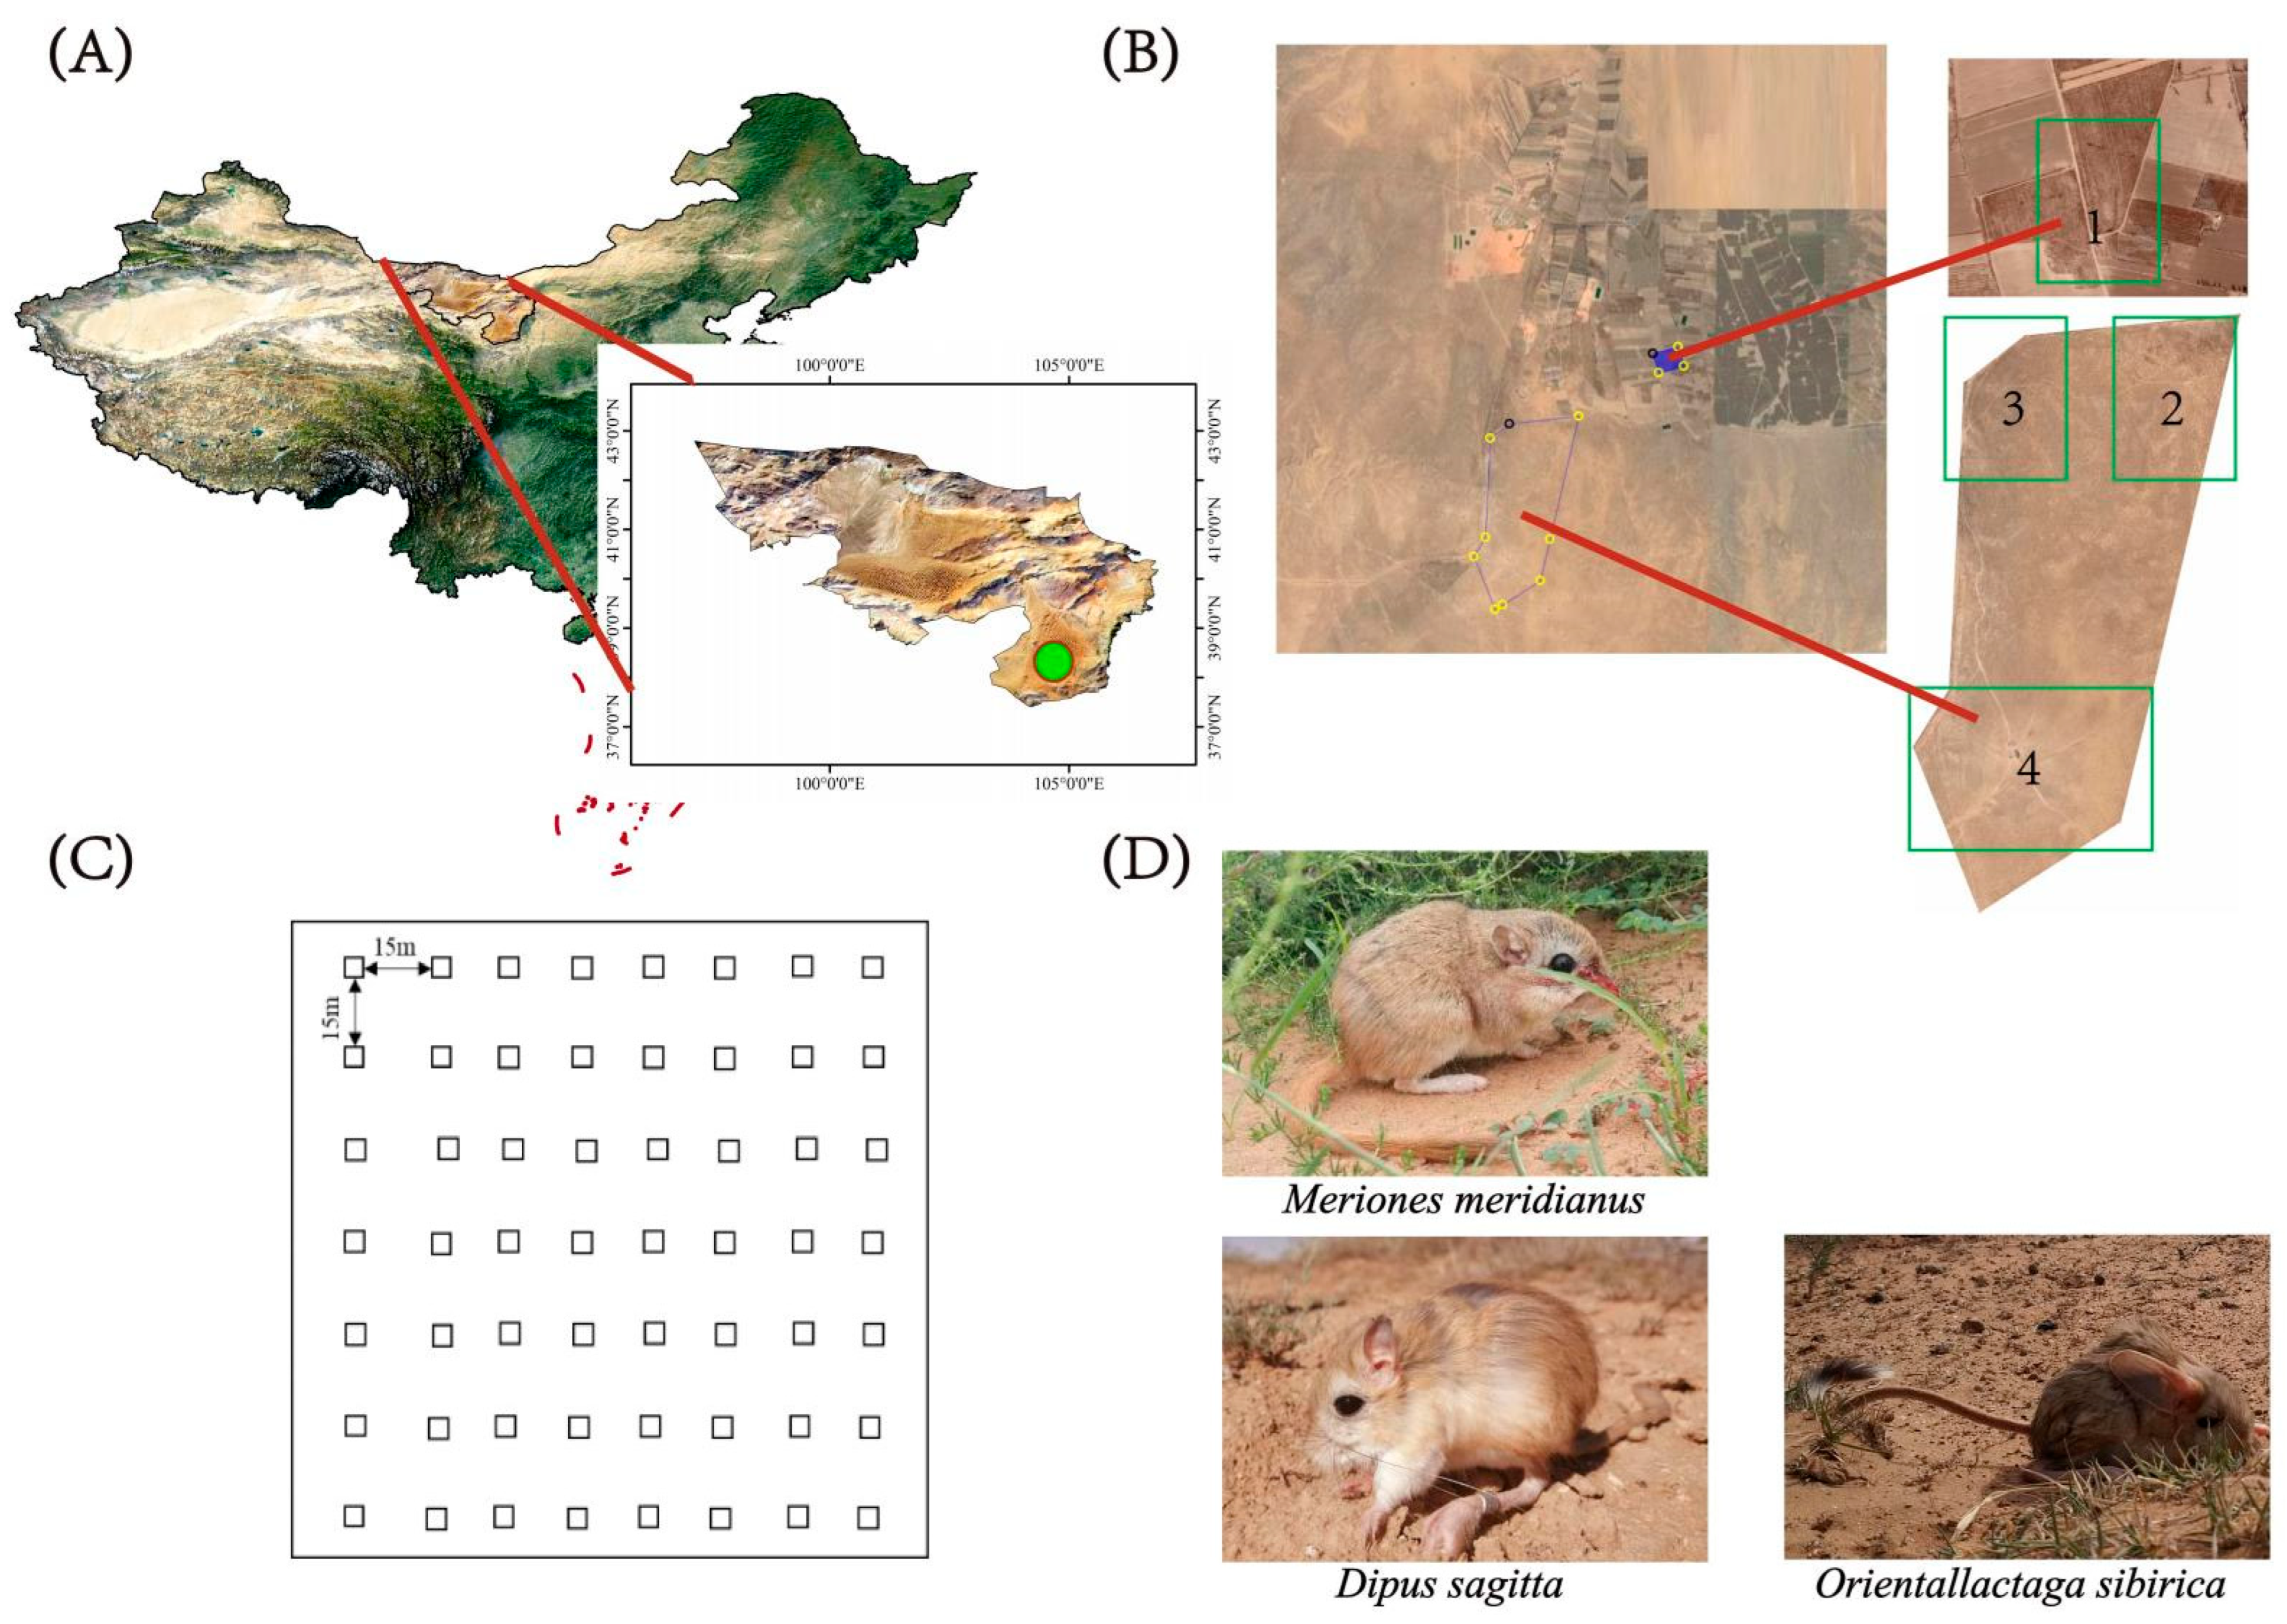
This study was carried out in the southern segment of the Alxa Desert, located in Inner Mongolia, China (104°10′–105°30′ E, 37°24′–38°25′ N) (Figure 1A). The research region features a continental climate characterized by cold, arid winters and warm summers. Annual precipitation ranges between 75 mm and 215 mm, with approximately 70% occurring during the period from June to September. The dominant soil types are gray desert soil and gray-brown soil. Vegetation cover is sparse, consisting primarily of xerophytic, super-xerophytic, and halophytic shrub species adapted to the arid environment. The experimental plots are located in a region severely disturbed by human activities, representing a typical agropastoral ecotone (Figure 1A).
Figure 1.
Selection and description of experimental plots. (A) Geographic location of the experimental area: Alxa Desert, Inner Mongolia, China (arid desert region). (B) Experimental plot design: 1 = reclamation-disturbed plots, 2 = grazing-excluded plots, 3 = rotational grazing-disturbed plots, 4 = overgrazing-disturbed plots. Three replicates were set for each plot type, totaling 12 plots. (C) Spatial distribution of live traps per plot. (D) Dominant rodent species in the experimental area.
Twelve typical plots were selected in the southern desert area of Alxa Left Banner, a region subjected to human disturbances including grazing and land reclamation. These plots consisted of three reclaimed plots (Figure 1(B1)), three grazing-excluded plots (Figure 1(B2)), three rotational grazing plots (Figure 1(B3)), and three overgrazed plots (Figure 1(B4)). Each plot covered an area of 60 ha, with an inter-plot distance exceeding 1 km. Field surveys were conducted annually from 2014 to 2020, spanning spring (April, May, and June), summer (July and August), and autumn (September and October), and all plots were surveyed during each sampling period.
2.2. Data Collection
2.2.1. Rodent Data Collection
To capture rodent individuals, a 7 × 8 trapping grid (1 ha) at a 15 m inter trap distance was established at the center of each 60 ha plot (Figure 1C). We placed one wire-mesh live trap (42 cm × 17 cm × 13 cm, Guixi Rodent Equipment Co., Ltd., Guixi, Yingtan, China) at each grid intersection (henceforth, trap station). A total of 56 live traps were deployed per plot. The traps were baited with fresh peanuts and checked twice (morning and afternoon) each day. The survey was conducted continuously for four consecutive days. We recorded the species and capture location of each trapped individual. Each captured animal was implanted subcutaneously with a passive integrated transponder (PIT) tag (2.12 mm × 8 mm; Guangzhou Ruimai Intelligent Technology Co., Ltd., Guangzhou, China) engraved with a unique identification (ID) number. To shield trapped rodents from disturbances caused by rainfall and other unforeseen events, a wooden shelter (15 cm × 10 cm × 10 cm) was placed inside each live trap to provide protection upon their entry. Meriones meridianus, Dipus sagitta and Orientallactaga sibirica are the dominant small mammal species. Natural enemies include Bubo bubo, Vormela peregusna, and Vulpes corsac (Figure 1D).
2.2.2. Environmental Factor Data Collection
Vegetation sampling: We randomly selected three 100 m2 plots within each unit to sample shrubs in each season. Within each 100 m2 plot, we randomly placed three 1 m2 quadrats to sample grasses and forbs. We measured the height, cover, density, abundance, and biomass of shrubs and herbs.
Soil sampling: At the same time as plant sampling, soil data were collected, including soil moisture content and soil hardness at 0–5 cm, 5–10 cm, 10–15 cm, and 15–20 cm. The soil hardness was measured using a soil hardness meter (TYD-2, Zhejiang Top Yunnong Technology Co., Ltd., Hangzhou, China), and the soil moisture content was determined by drying the samples at 105 °C for 8 h.
Meteorological sampling: The meteorological data were obtained from the “Luan-jingtan Meteorological Station in Alxa League,” which is 5.95 ± 0.34 (Mean ± SE) km away from the study area. The meteorological data include the average monthly precipitation, average annual precipitation, monthly average relative air humidity (%), average air temperature (°C), sunshine duration (h), annual mean temperature, monthly mean temperature, average overwintering temperature, annual average sunshine hours, and total annual radiation during the period 2014–2020.
2.3. Statistical Analyses
To examine differences in rodent community characteristics across different years and habitat patches under varying disturbance regimes, we analyzed the following metrics using a nonlinear mixed-effects model to eliminate the temporal effect induced by long-term scales: plant metrics under different disturbances, the capture proportion of each rodent species within the same disturbance type, total rodent capture rates under different disturbances, and diversity indices. The main comparison objects were set as fixed factors, while other factors were treated as random factors.
To investigate the seasonal patterns and interannual fluctuations of the metacommunity in the study area, a two-way analysis of variance (ANOVA) was conducted on total capture rates and community abundance with year and month as the fixed factors. Additionally, to explore how year and disturbance effects influence rodent communities, one-way ANOVA was separately implemented on rodent abundance and diversity indices in plots under different disturbance regimes. A Tukey test was performed for multiple comparisons of means of diversity indices. All difference analyses were performed using SAS 9.4 software with a significance level set at α = 0.05. Unless otherwise specified, all values are presented as mean ± 1 standard error of the mean.
2.4. Diversity Index in Metacommunity
We used 6 indicators to estimate the variation characteristics of rodent community diversity, including species richness (S), Shannon–Wiener diversity index (H), Simpson diversity index (D), evenness index (E), In this study, beta diversity was calculated based on the Sørensen dissimilarity index (a core metric in research on β-diversity of biological communities, quantifying the relative contributions of “species turnover” and “nestedness” to community dissimilarities, βSOR) and Cody similarity index (a metric for measuring the similarity of community species composition). The Sørensen dissimilarity index was further partitioned into two components: spatial species turnover (or replacement, βSIM) and nestedness of species assemblages (βSNE).
Based on the distribution of sample plots and vegetation characteristics in the study area, this study comprehensively considers the degree of interference and landscape fragmentation and divides the habitat gradient in the study area according to the order of Area1 (grazing-excluded plots) → Area2 (rotational grazing plots) → Area3 (overgrazed plots) → Area4 (reclaimed plots).
We used 5 indicators to estimate habitat productivity and ‘concealment’, including average height, density of shrub, average coverage of shrub, coverage of shrub, and plant biomass. The measurement accuracy is 0.01 g. The determination of grass indicators includes the average height (cm), density (plants/m2), and dry weight (accuracy 0.01 g) of grasses in a 1 m2 quadrat.
2.5. Response Mechanism Verification Method
Structural equation modeling (SEM) offers four key advantages: I. It can handle multiple dependent variables simultaneously; II. It allows for measurement errors in both independent and dependent variables; III. It enables concurrent evaluation of factor structures and inter-factor relationships; IV. It provides multiple goodness-of-fit indices to assess the overall model fit. Therefore, SEM empowers ecologists to test complex multivariate hypotheses regarding ecosystems, overcoming the limitations of traditional univariate hypothesis-testing frameworks in studying interdependent systems. The SEM was employed to analyze the response relationships between the characteristics of rodent local communities and metacommunities, and climatic, edaphic, and vegetation characteristics. Two-stage modeling was used to construct the final model. In the first stage, Confirmatory Factor Analysis (CFA is a statistical method used to verify whether a pre-specified factor structure fits the actual data) was employed to determine the goodness-of-fit of the factor structure. Climate, vegetation, and soil characteristics, which cannot be directly measured, were set as latent variables, while the measured meteorological and environmental factors were treated as observed variables. The second stage was structural model fitting. The maximum likelihood (ML) method was used for parameter estimation [25]. Chi-square degree of freedom ratio, Root Mean Square Error of Approximation (RMSEA), Non-Normed Fit Index (NNFI), and Comparative Fit Index (CFI) were used to test the goodness of fit. RMSEA less than 0.1 indicates a good fit, and the smaller the value, the better fit the model. The closer NNFI and CFI are to 1, the better the model is. The relationship between the latent variable and the measurement index is expressed by the factor load. The relationship between latent variables is expressed by the regression coefficient. All path coefficients are solved using complete standard solution. The analysis of all structural equation models was performed using SPSS AMOS 23.0.
3. Results
3.1. Rodent Community Structure
From 2014 to 2020, a total of 129,024 trap-days of live traps were deployed in the study area, resulting in 9686 capture events and the successful capture of 4208 rodent individuals. These individuals belonged to 10 species across three families:
Cricetidae (five species): Meriones meridianus, Rhombomys opimus, Phodopus roborovskii, Cricetulus barabensis, and Cricetulus eversmanni.
Dipodidae (four species): Dipus sagitta, Orientallactaga sibirica, Stylodipus andrewsi, and Salpingotus crassicauda.
Sciuridae (one species): Spermophilus alaschanicus.
Notably, rare captures of four species were recorded: one S. crassicauda in the overgrazed plot in 2015; two C. barabensis (one in the ungrazed plot in 2016 and one in the cultivated habitat in 2017); four R. opimus in the ungrazed plot in 2014; and three C. eversmanni in the cultivated plot during 2019–2020. Due to their extremely low abundances, these four species were classified as rare species and thus excluded from the calculations of capture rates and community species diversity indices.
In this study, the rodent communities were categorized into two levels: (1) local rodent communities, which refer to those within each habitat patch generated by different disturbance regimes; and (2) the metacommunity, defined as an assemblage of 4 types (12 total) of local communities connected through species dispersal.
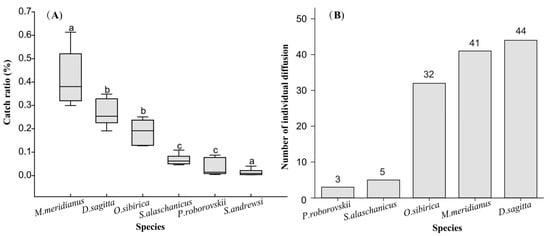
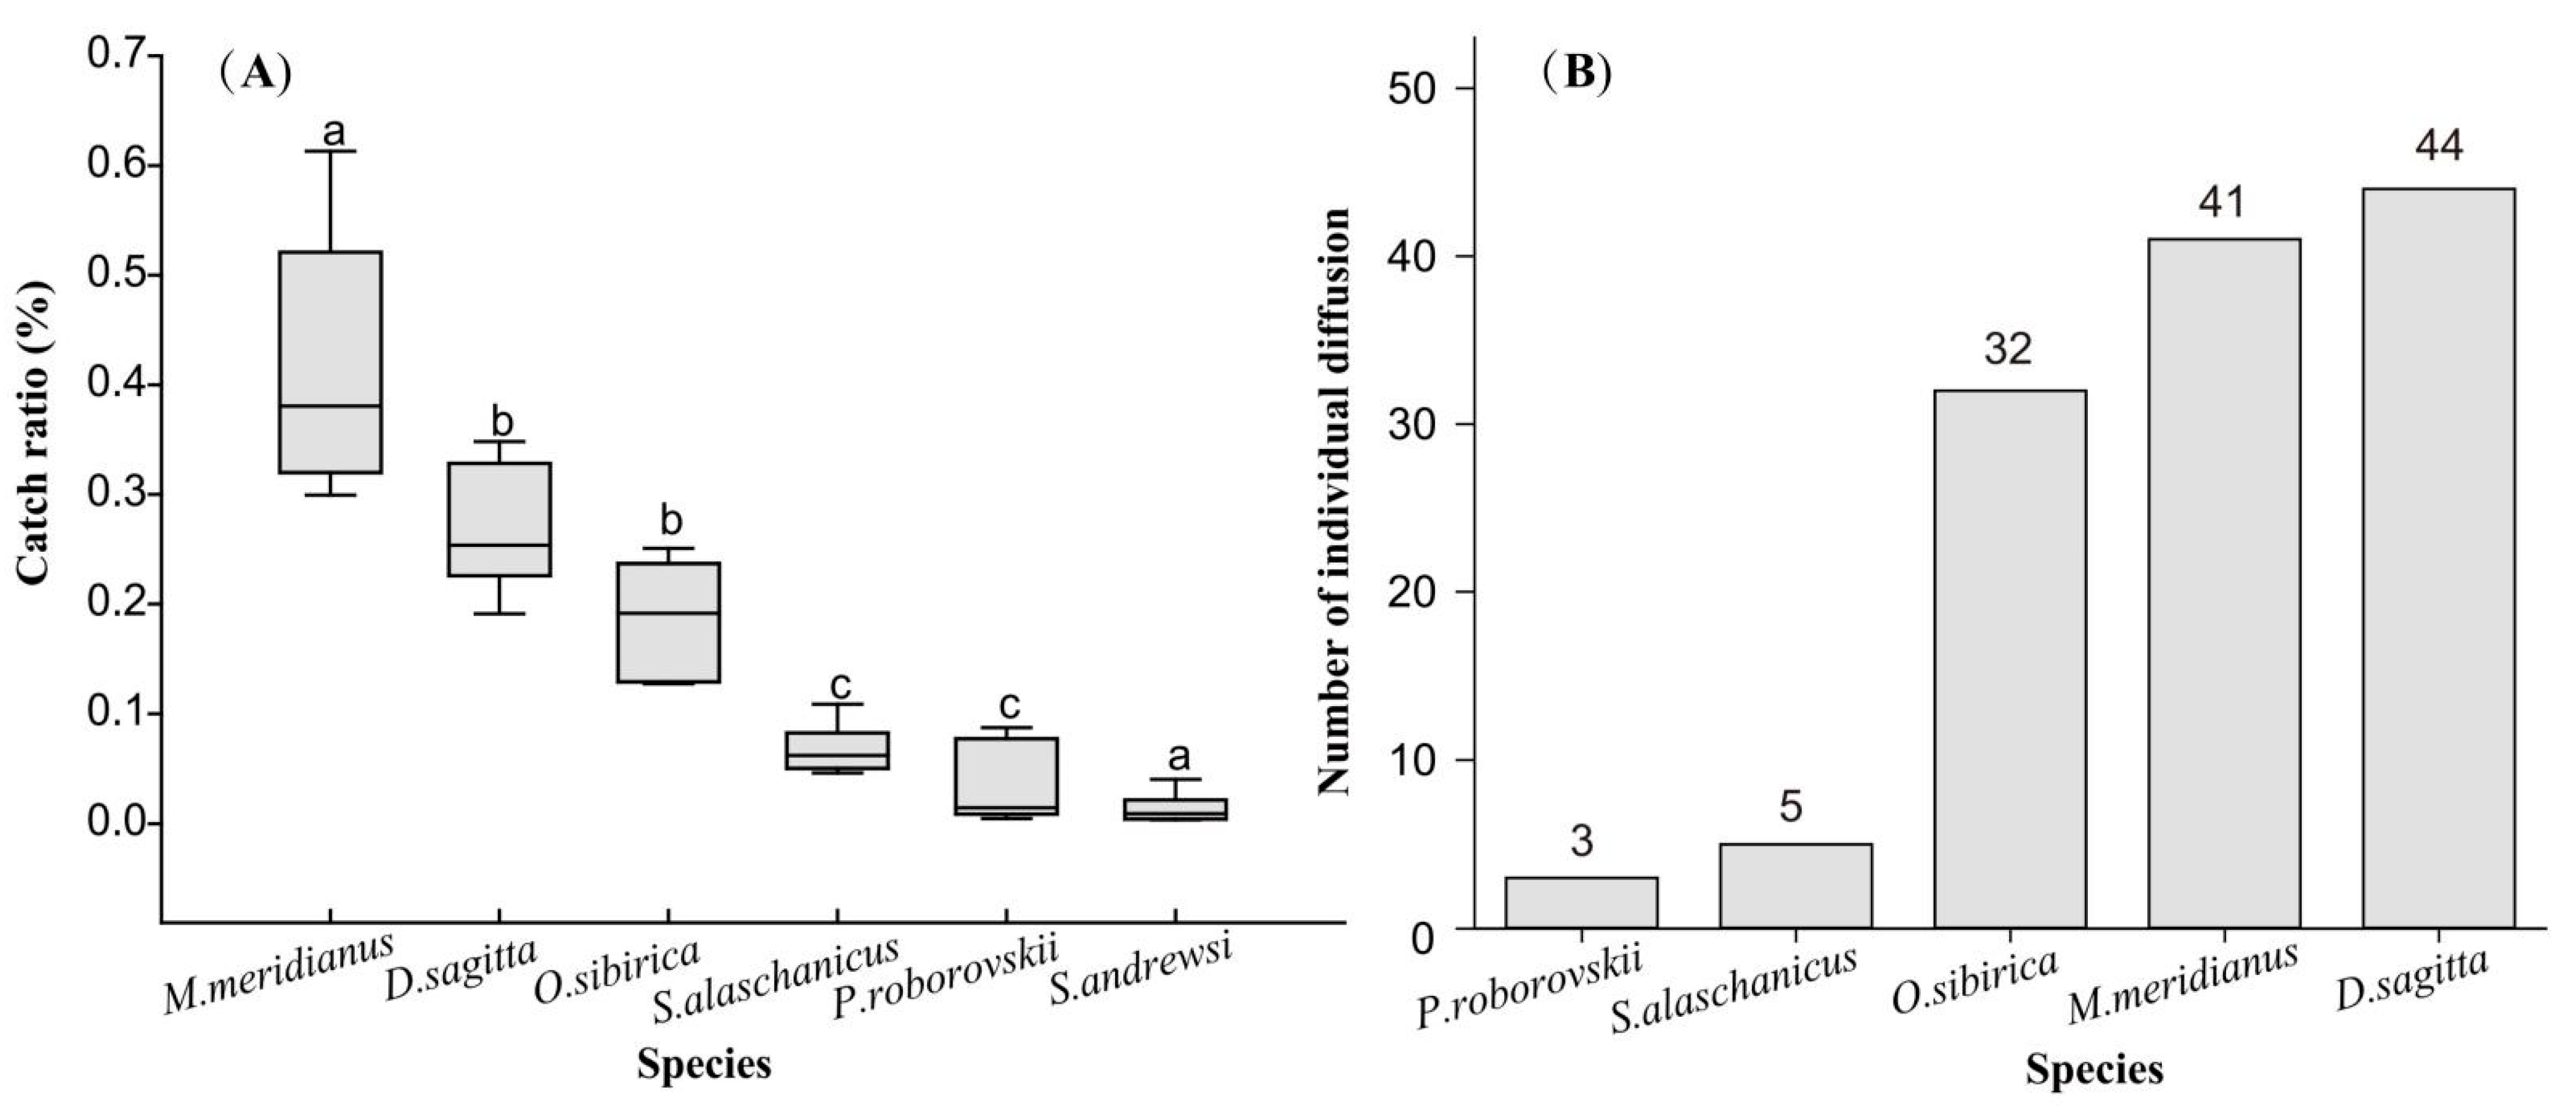
A mixed linear model was used, with the year as the fixed factor, and the disturbance condition and the number of plot replicates as the random factors, to calculate the differences in capture rates among species. Species composition in the aggregated communities from 2014 to 2020 indicated significant differences in the proportion of catches among different rodent species (F = 51.057, p < 0.0001). The proportion of catches of M. meridianus was significantly higher than that of other mouse species; the proportion of catches of D. sagitta and O. sibirica was significantly higher than that of S. alaschanicus, S. andrewsi, and P. roborovskii (Figure 2A). To verify the individual dispersal phenomenon of the rodent metacommunity in the study area, this paper counted the dispersal of rodent individuals among different habitat patches during the research period. From 2014 to 2020, a total of 125 rodent individuals diffused between different patch habitats within the study area, with a total of 206 diffusion events occurring (Table 1). The numbers corresponding to the intersections of different habitats in the table represent the number of rodent diffusion events, including diffusion events within the same disturbed habitat but across different patch habitats, as well as between different disturbed habitats. The rodent species involved in the diffusion mainly included M. meridianus (41 individuals), D. sagitta (44 individuals), and O. sibirica (32 individuals), accounting for 93.6% of the total diffusing individuals (Figure 2B). Among the plots under different grazing regimes, the three overgrazing replicates showed the highest frequency of dispersal events (S9–S7: 52, S9–S8: 33, S8–S7: 13), with O. sibirica as the dominant species therein. The three rotational grazing replicates ranked second in the occurrence of dispersal events (S6–S5: 17, S5–S4: 15, S6–S4: 14), where D. sagitta and M. meridianus were the main taxa. Notably, compared with gerbils, jerboas characterized by bipedal saltatory locomotion exhibited superior dispersal capacity (Table 1).
Figure 2.
Species composition (A) and individual dispersal (B) of metacommunity, Alxa Desert, Inner Mongolia, China. Different lowercase English letters in the figure indicate significant differences in the proportion of catches among different mouse species (p = 0.05).
Table 1.
Individual dispersal events among different habitats in the aggregation community, Alxa Desert, Inner Mongolia, China.
3.2. Alpha Diversity of Rodent Communities
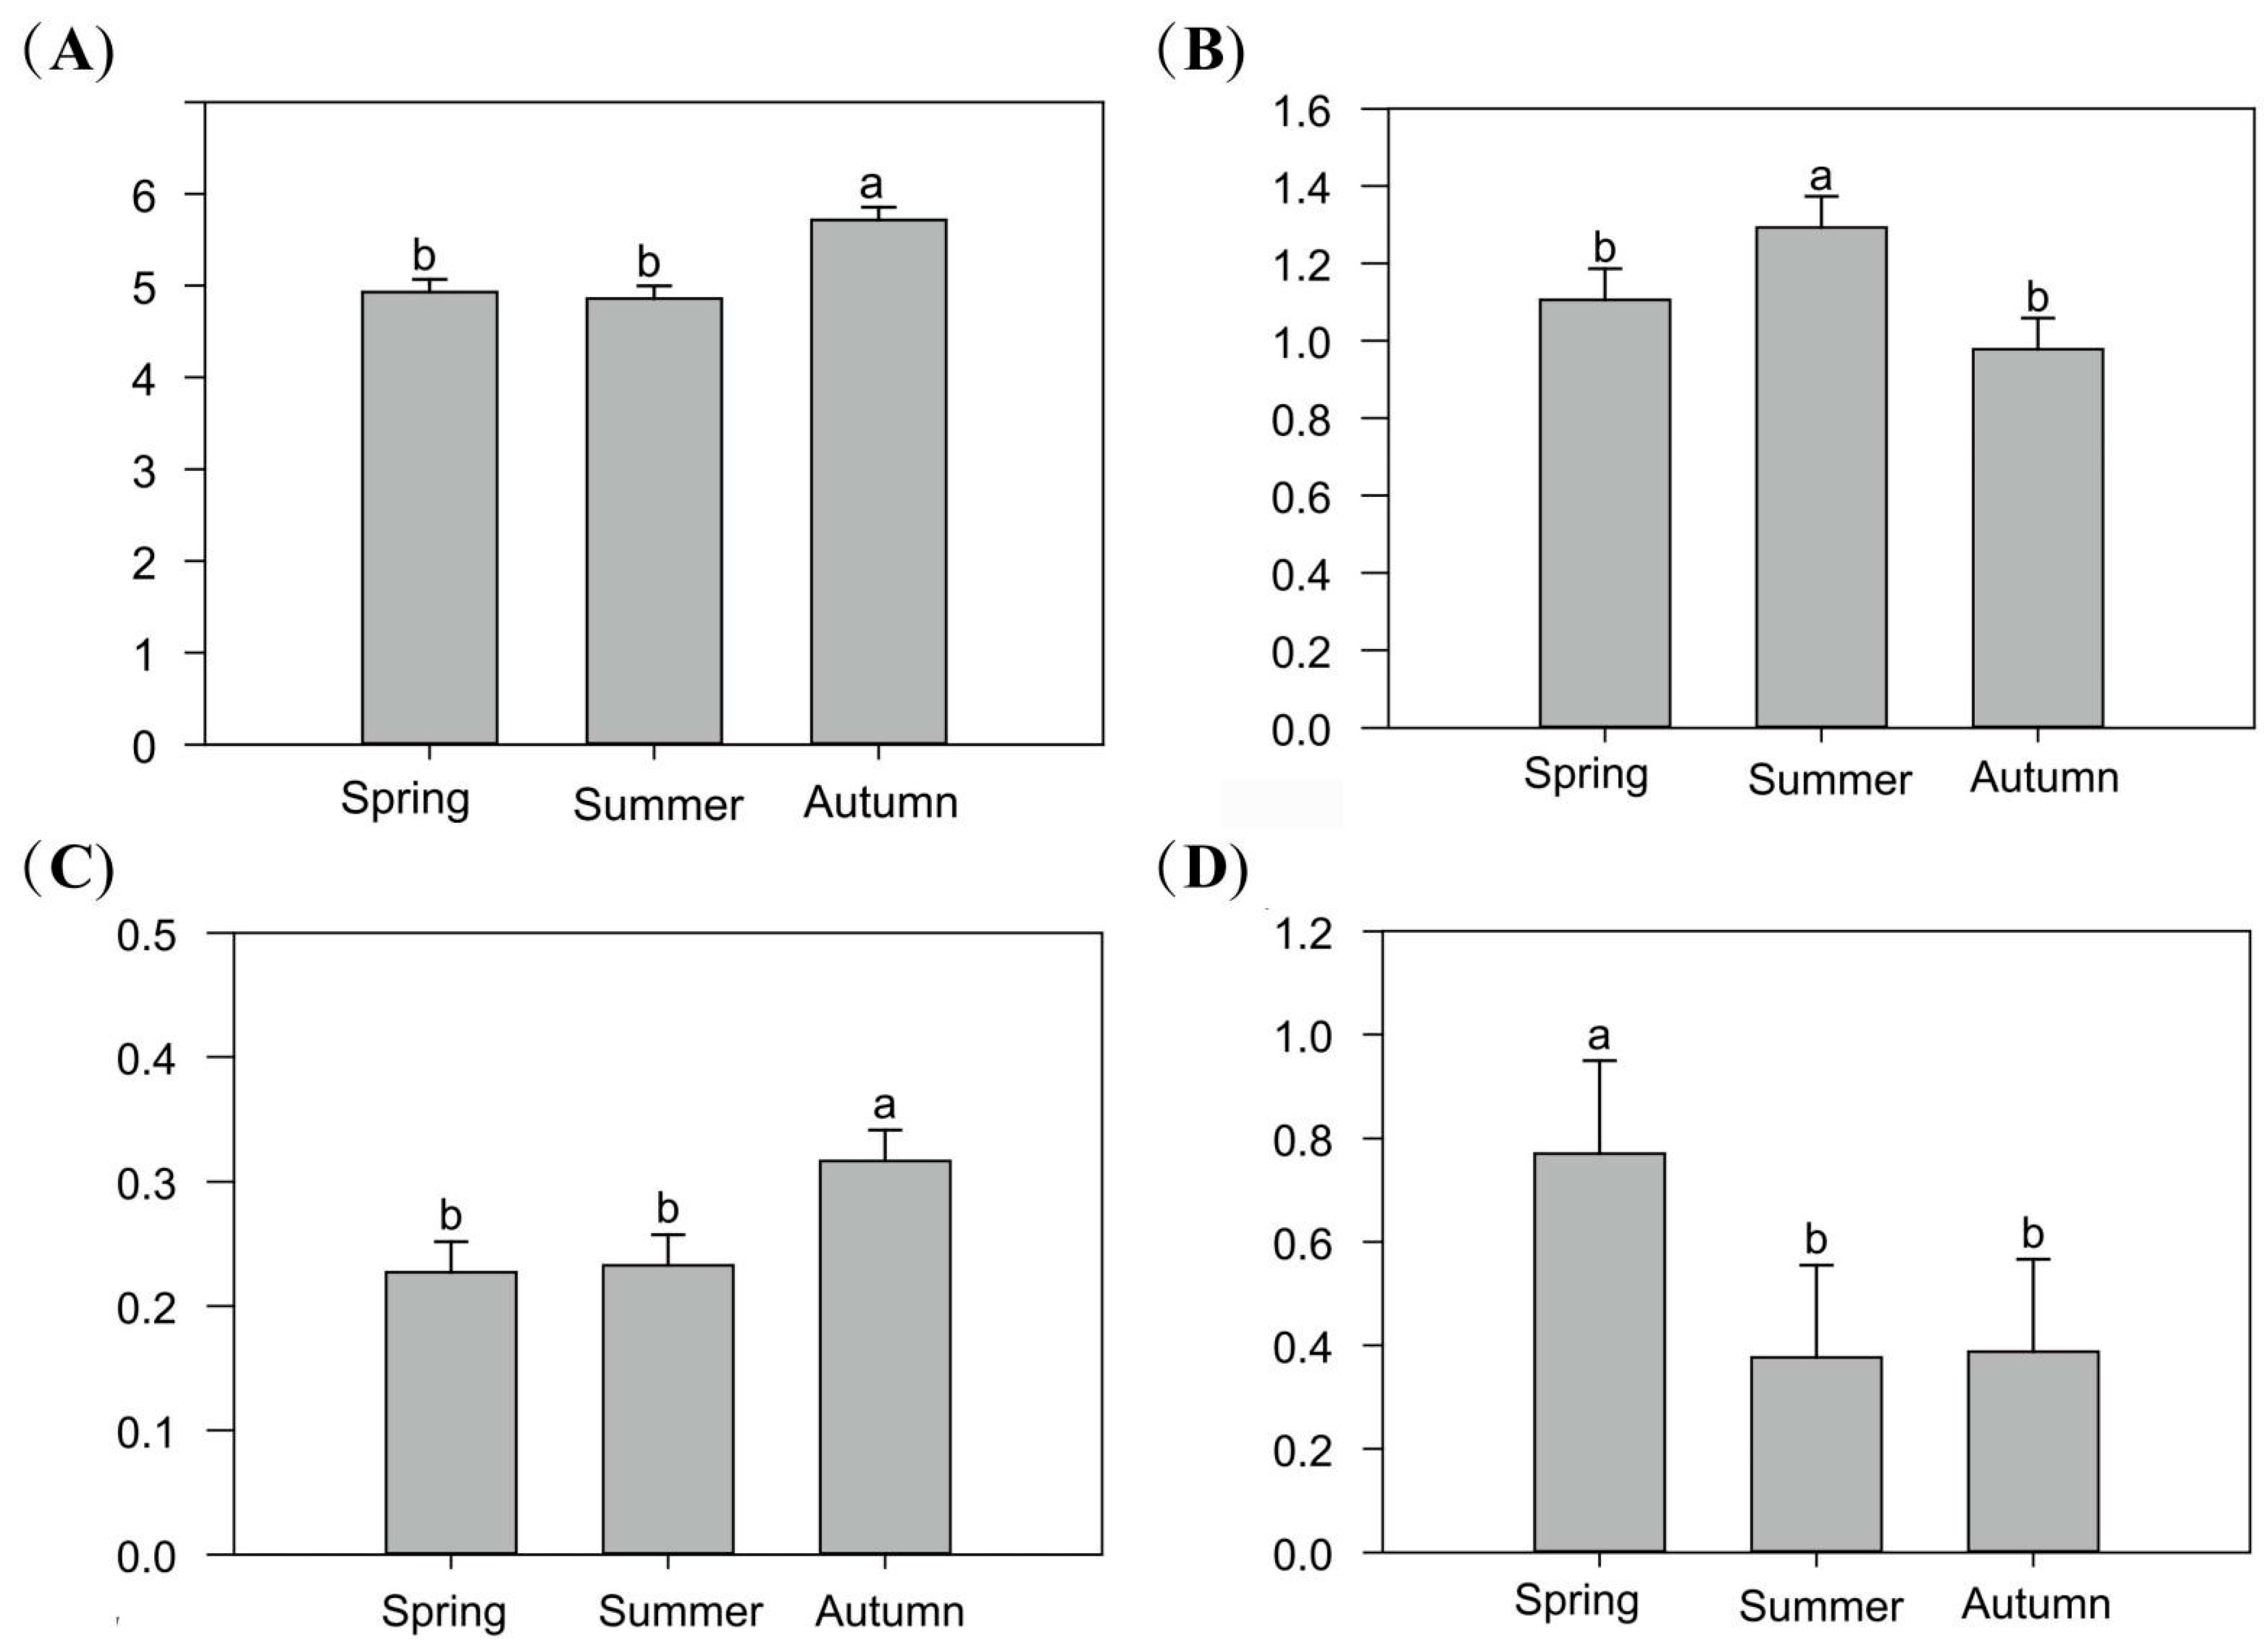
A mixed linear model was adopted, with seasons set as fixed factors, and interannual variation, disturbance conditions, and the number of plot replicates set as random factors, to calculate the differences in species richness. From 2014 to 2020, species richness (S) of the metacommunity was significantly higher in autumn than in spring and summer (F = 15.95, p < 0.0001), while there was no significant difference between summer and spring (Figure 3A). The Shannon–Wiener diversity index of the metacommunity showed significant seasonal differences, with species diversity being significantly higher in summer than in spring and autumn (F = 13.99, p < 0.01) (Figure 3B). The Simpson diversity index of the metacommunity was significantly higher in autumn than in summer and spring (F = 15.02, p < 0.001) (Figure 3C), while there was no significant difference between spring and summer. The Pielou evenness index of the metacommunity was significantly higher in spring than in summer and autumn (F = 9.27, p < 0.001) (Figure 3D).
Figure 3.
Temporal (season) pattern of α diversity in the rodent metacommunity, Alxa Desert, Inner Mongolia, China. (A) is the seasonal variation of species richness, (B) is the seasonal variation of Shannon–Wiener diversity index, (C) is the seasonal variation of Simpson diversity index, (D) is the seasonal variation of Pielou evenness index. Different lowercase English letters in the figure indicate significant differences in the proportion of catches between different seasons (p = 0.05).
3.3. Beta Diversity of Rodent Communities
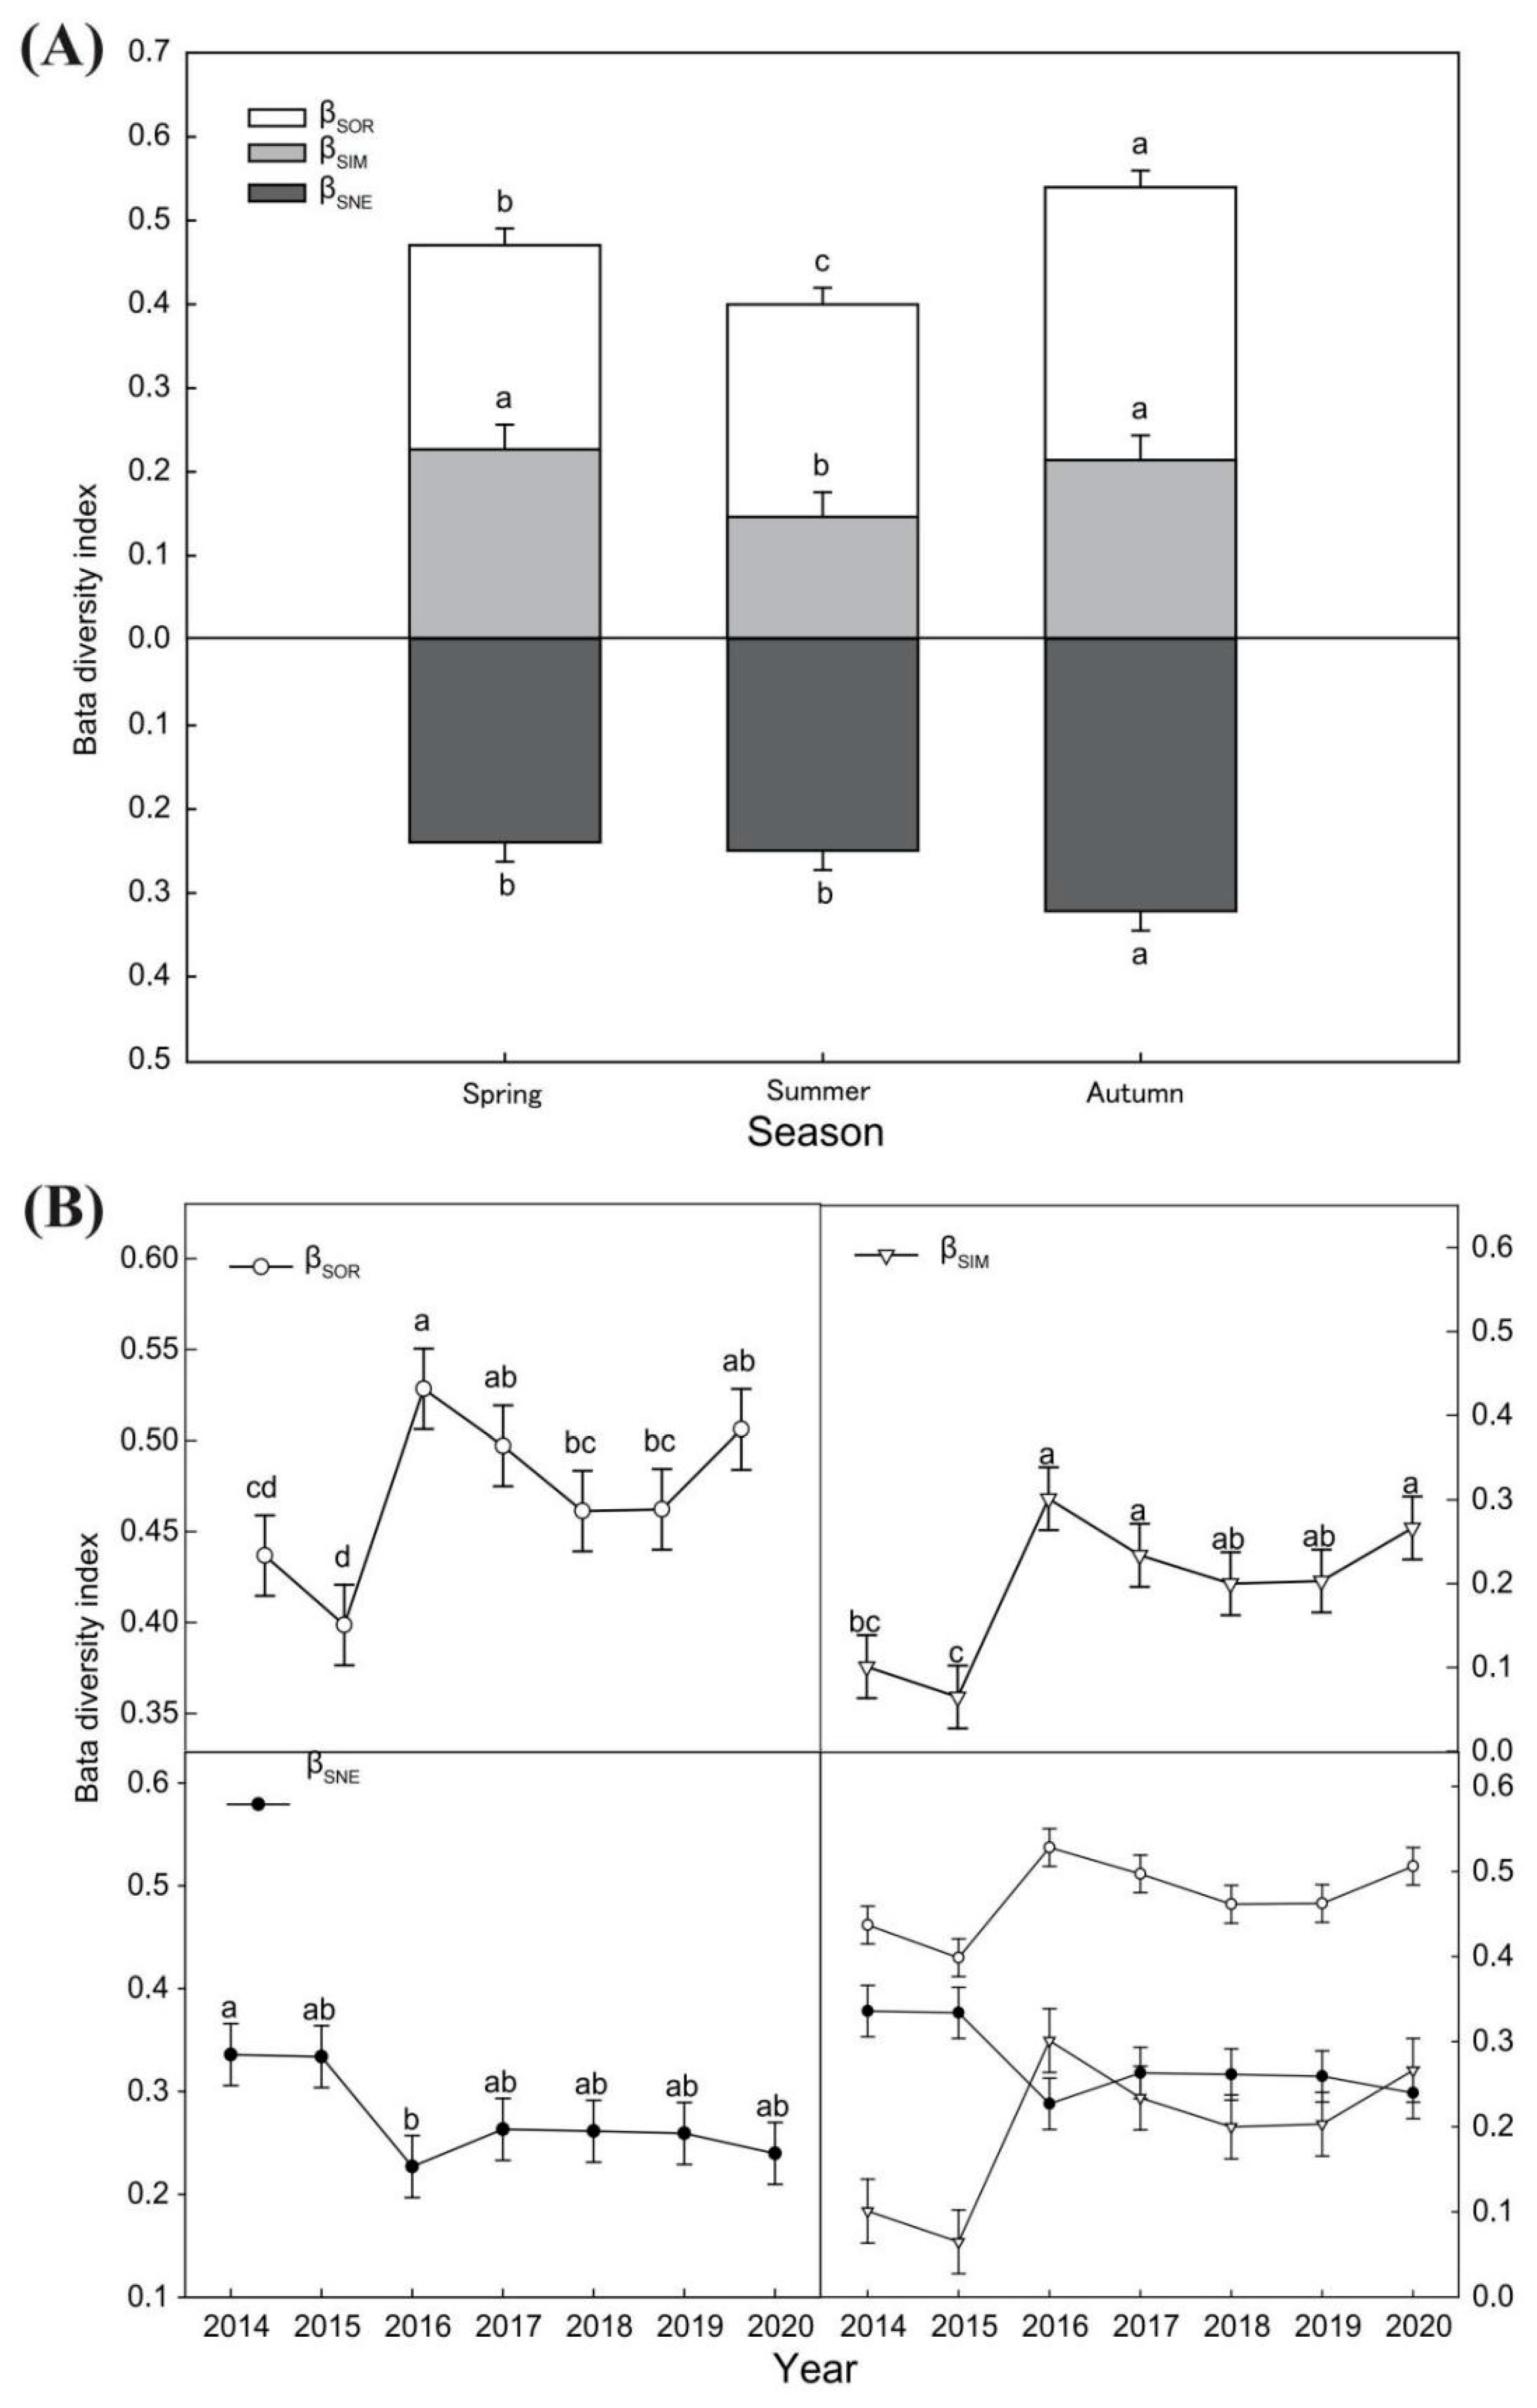
An analysis of variance was conducted on the β diversity of metacommunities from 2014 to 2020, considering year, season, and their interaction. The results indicated that the βSOR index, βSIM, and βSNE of metacommunities were all influenced by year, month, and their interaction (Table 2). The βSOR index in autumn was significantly higher than in spring, while the βSOR index in spring was significantly higher than in summer. The βSIM index in both spring and autumn was significantly higher than in summer. However, there was no significant difference between spring and summer. The βSNE index in autumn was significantly higher than in summer and spring, while there was no significant difference between summer and spring.
Table 2.
Two-way ANOVA analysis of beta diversity in aggregated communities, Alxa Desert, Inner Mongolia, China.
From 2014 to 2020, there were significant differences in the β diversity indices (βSOR, βSIM, βSNE) of the metacommunity across the years (Figure 4). The βSNE index showed the most dramatic inter-annual variation. βSOR generally exhibited an upward trend year to year, with a significant increase in 2016 compared to all other years except 2017 and 2020. βSIM demonstrated significant increases in 2016, 2017, and 2020 compared to 2014 and 2015, with no significant differences between other years. The βSNE index generally showed a decreasing trend, with a significant increase in 2014 compared to 2016, while there were no significant differences between other years. In the study period, the βSIM and βSNE indices alternated in dominating the species distribution pattern of the metacommunity, with βSIM < βSNE only in 2016 and 2020, and βSNE > βSIM in all other years.
Figure 4.
Temporal (season (A) and year (B)) pattern of β diversity in the rodent metacommunity, Alxa Desert, Inner Mongolia, China. Different lowercase English letters in the figure indicate significant differences in the proportion of catches between different seasons and years (p = 0.05). (B) represents βSOR, βSIM, βSNE, and the β-diversity of the metacommunity, respectively.
3.4. Responses of Local Rodent Communities to Fluctuations in Environmental Factors
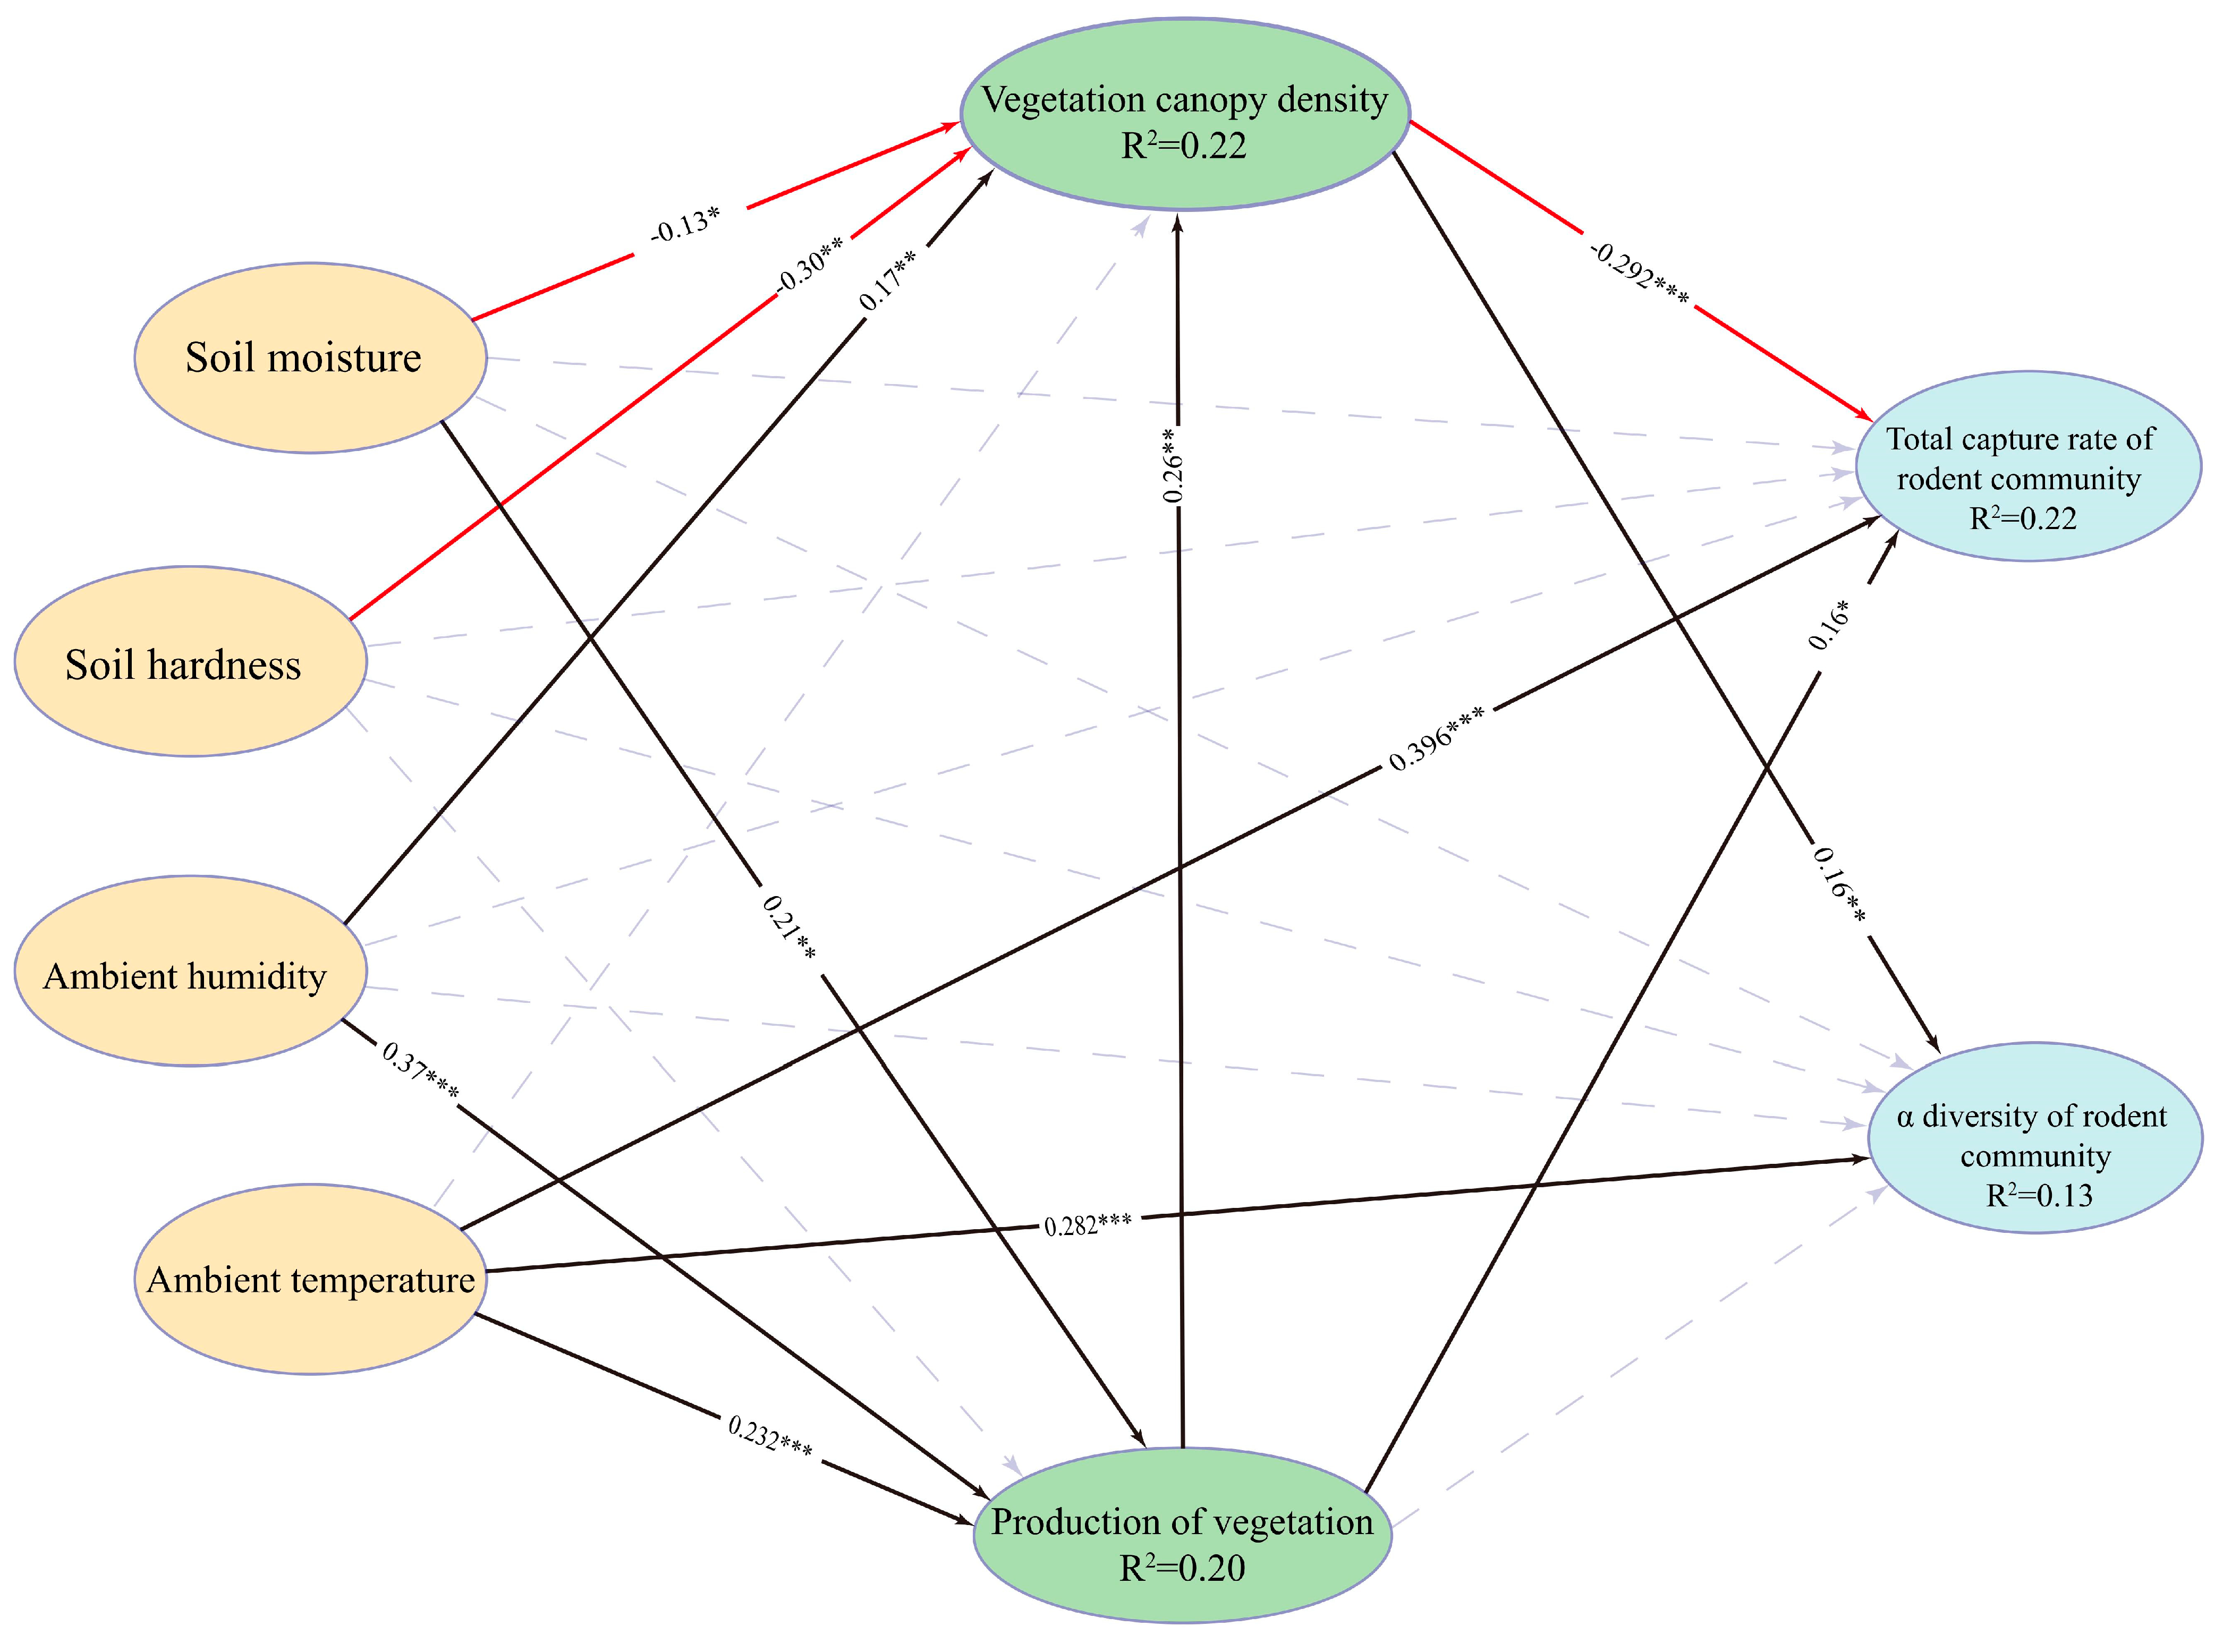
Temperature had a significant impact on the community abundance (path coefficient: 0.396, p < 0.001) and the Shannon–Wiener diversity index of local rodent communities (path coefficient: 0.282, p < 0.001). Additionally, temperature had a significant positive impact on the number of individuals in local rodent communities by significantly enhancing vegetation productivity (path coefficient: 0.232, p < 0.001) (path coefficient: 0.16, p < 0.05). Soil moisture content, soil hardness, and water content had no direct impact on the rodent community characteristics. They indirectly affect rodent community characteristics by influencing vegetation canopy density and grassland productivity. Precipitation (exogenous latent variable water) exerted a negative effect on rodent communities by increasing vegetation canopy density (path coefficient: 0.17, p < 0.01), while positively affecting faunal community diversity (path coefficient: 0.16, p < 0.001). Both the aboveground biomass and canopy density of vegetation had a direct impact on rodent communities. Soil hardness and soil moisture content, on the other hand, indirectly affected rodent community characteristics through vegetation characteristics. Similarly, water conditions did not have a direct impact on rodent communities but indirectly affect them through vegetation characteristics. Soil moisture content positively affected the total number of individuals in the animal community by influencing canopy density (path coefficient −0.13, p < 0.05), thereby reducing community diversity. It also positively impacted the animal community by increasing grassland productivity (path coefficient 0.21, p < 0.01). Soil hardness only influenced the total number of individuals and community diversity in the rodent community by affecting canopy density (path coefficient −0.30, p < 0.01), promoting and reducing these characteristics, respectively (Figure 5).
Figure 5.
Path diagram of latent variable relationships in rodent local communities in Alxa Desert, Inner Mongolia, China. In the figure, yellow represents environmental factors, green represents plant factors, and blue represents animal factors. The values adjacent to the arrows in the figure represent correlation coefficients (r). The “-” symbol indicates a negative effect, and asterisks denote significant effects: * p < 0.05, ** p < 0.01, and *** p < 0.0001. The dashed line indicates that the impact has not reached a significant level (r = 0.05).
3.5. Responses of Metacommunity to Fluctuations in Environmental Factors
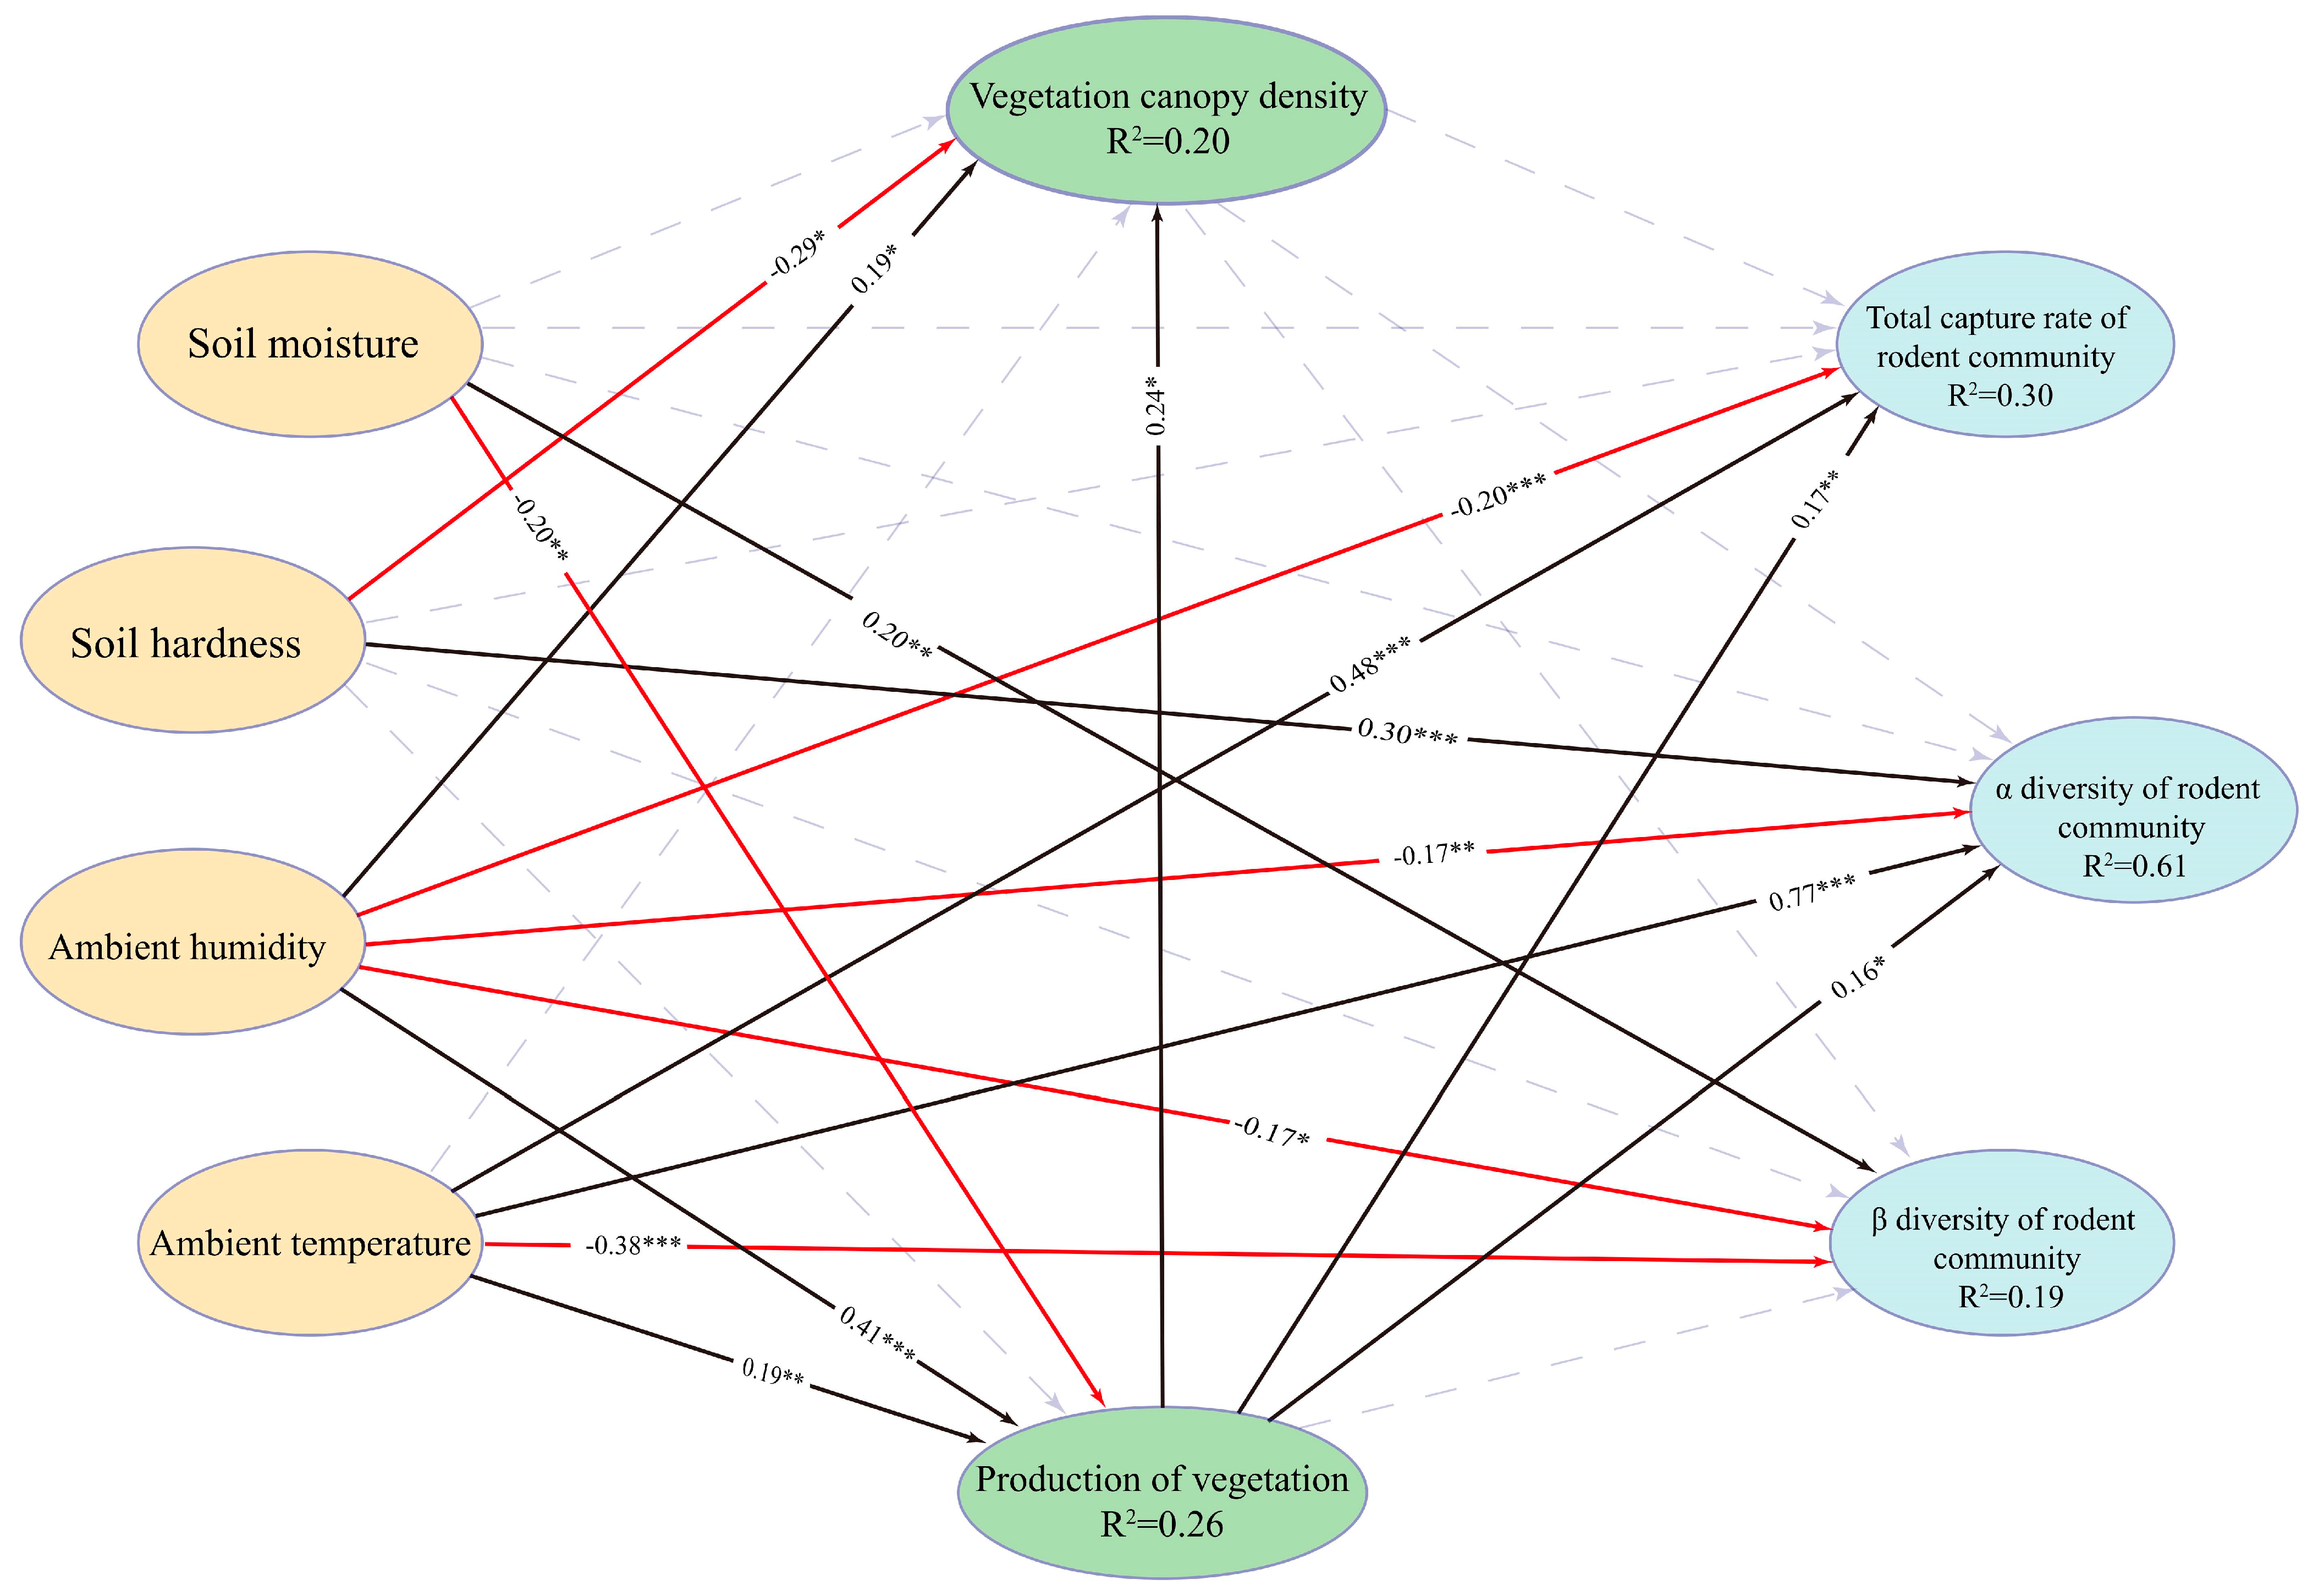
Soil moisture content had a significant positive effect on the β diversity of rodent communities (path coefficient: 0.20, p < 0.01) but had no effect on the total number of individuals and α diversity of the communities. At the same time, it indirectly exerted a positive influence on the total number of individuals in rodent communities (path coefficient: 0.17, p < 0.01) through the aboveground productivity of vegetation (path coefficient: 0.20, p < 0.01). Soil hardness had a direct positive effect on the α diversity of rodent communities (path coefficient: 0.30, p < 0.001).
In the structural equation model, was moisture composed of monthly average precipitation and relative humidity. Moisture exhibited a high factor loading on both measurement variables, indicating that these variables had a significant impact on both rodent communities and plant communities (Figure 6). Moisture exerted a direct negative effect on the total individual count (path coefficient: −0.20, p < 0.001), β diversity (path coefficient: −0.17, p < 0.01), and α diversity (path coefficient: −0.17, p < 0.001) of rodent communities. Simultaneously, it indirectly positively influenced the total individual count and α diversity of the communities by affecting the above-ground productivity of vegetation (path coefficient: 0.41, p < 0.001).
Figure 6.
Path diagram of latent variables in the whole model of rodent metacommunity, Alxa Desert, Inner Mongolia, China. In the figure, yellow represents environmental factors, green represents plant factors, and blue represents animal factors. The values adjacent to the arrows in the figure represent correlation coefficients (r). The “-” symbol indicates a negative effect, and asterisks denote significant effects: * p < 0.05, ** p < 0.01, and *** p < 0.0001. The dashed line indicates that the impact has not reached a significant level (r = 0.05).
Latent variable temperature was primarily composed of average temperature, average maximum temperature, and average minimum temperature. The model indicated that temperature had a positive impact on the total number of individuals in the assemblage community (path coefficient of 0.48, p < 0.001) and α diversity (path coefficient of 0.77, p < 0.001), while it exerted a negative effect on community β diversity (path coefficient of −0.38, p < 0.001). Additionally, temperature positively influenced the total number of individuals and α diversity in the community through above-ground vegetation productivity (path coefficient of 0.19, p < 0.01) (Figure 6).
4. Discussion
4.1. Impact of Fluctuations in Climatic Conditions on Rodent Communities
Small rodents are key indicator organisms for habitat stability, biodiversity, and utilization pattern changes [14], as they rapidly respond to environmental changes, disturbances, and subsequent habitat succession or fragmentation [15,16]. Their occurrence, population density, community diversity, and morphological traits are practical tools for evaluating ecosystem health [17]. Structural equation models (SEM) have been widely used to explore relationships between animal assemblages and climatic fluctuations, revealing direct/indirect effects of climate variables on species distribution, population dynamics, interspecific interactions, and ecosystem functions [26,27,28].
Water and heat are the primary limiting factors in desert ecosystems. This study confirmed that temperature and precipitation fluctuations, along with pulse effects of extreme climate events, exert profound impacts on desert rodent communities—consistent with previous findings that climate change significantly affects species distribution, richness, and diversity [12,13]. Specifically, temperature exerted a direct positive effect on community individual numbers and an indirect positive effect by promoting grassland productivity. Precipitation showed no direct impact on local community habitat characteristics but indirectly affected community abundance: it increased abundance via elevated aboveground productivity yet reduced individual numbers by increasing vegetation canopy density. At the metacommunity scale, precipitation had a direct negative effect and an indirect positive effect on total individuals and α-diversity through enhanced aboveground productivity. These results indicate that water and temperature affect rodent communities through similar pathways, but metacommunity responses are more diverse, highlighting the predominant large-scale impact of climatic fluctuations on animal communities.
Species dispersal, a core process in metacommunity dynamics [29,30], mediates community structure. Our 7-year monitoring recorded numerous inter-habitat rodent dispersal events, with D. sagitta having the highest dispersal frequency, followed by M. meridianus and O. sibirica. Phodopus roborovskii and S. alaschanicus only dispersed between patches in overgrazed habitats with short distances. Notably, despite M. meridianus having a significantly larger population than D. sagitta and O. sibirica, its dispersal number was lower. This suggests that dispersal is constrained not only by habitat characteristics, population density, and distance but also by individual traits—bipedal D. sagitta and O. sibirica have superior locomotor capacity, leading to more frequent dispersal. Additionally, no consistency was found between dispersal events and population density: 2019 had the highest metacommunity population but the lowest dispersal frequency, indicating that environmental and climatic factors have stronger impacts on dispersal than rodent density.
Climatic effects on rodents are modulated by disturbances, microhabitats, and species-specific adaptability [31]. Similar to Leanne et al. [32], who found North American grassland rodents respond to most climatic variables, our study showed Alxa Desert dominant rodents (D. sagitta, O. sibirica, M. meridianus) have divergent climatic adaptabilities—Dipodidae species are more temperature-adaptable, while Cricetidae are more rainfall-adaptable [33]. Unlike Richard et al. [34], who observed rainfall-induced resource pulses boosting Calomys musculinus populations in Argentine Pampas, Alxa Desert rainfall did not trigger food pulses for rodents but increased vegetation canopy density, negatively affecting open-habitat jerboas and benefiting canopy-preferring species. This aligns with Wu et al. [33], who reported vegetation biomass positively correlates with rodent abundance, while canopy density has a negative effect.
Overall, climatic factors act through two mechanisms: direct effects on populations and indirect effects via modifying vegetation canopy closure and productivity. Small-scale disturbances buffer climatic impacts, and heterogeneous responses of dominant species to disturbances and rainfall render local communities insensitive to rainfall variations. Short-term extreme climatic events may also affect species distribution and persistence, though such impacts remain underdetected and require further study.
4.2. The Mechanism Underlying How Fluctuations in Climatic Conditions Affect Rodent Community Diversity
Since the 1990s, with the increasingly prominent issue of climate change and widespread attention to biodiversity conservation, it has been recognized that climate fluctuations exert significant impacts on terrestrial vegetation, herbivores, and carnivores [35]. Over the past few decades, ecologists have dedicated efforts to exploring the relationships between biodiversity and ecosystem function, stability, and ecological services [36]. A growing body of experimental data confirms that biodiversity loss can impair and disrupt the stability of ecosystem functions [37]. Numerous studies have investigated the response of rodent community diversity loss to climate change, yet most focus on large-scale analyses.
Simone et al. found in their study of small mammal communities in Europe that heavy rainfall and low temperatures positively affect the abundance and richness of the Apodemus sylvaticus in the community, while extreme high temperatures are significantly negatively correlated with the Mus spretus [38]. Meanwhile, species loss (Crocidura russula) occurred in the community. A similar pattern was observed in this study: rodents such as M. unguiculatus (2014), Rhombomys opimus (2015), Salpingotus crassicauda (2016), and Cricetulus barabensis (2018) disappeared successively in the study area over the years, resulting in the loss of species diversity at both local and metacommunity scales. In our previous studies, these species once maintained relatively large population sizes; however, with the cumulative effects of anthropogenic disturbances and extreme weather events over the years, their capture rates have consistently declined.
Of course, other potential mechanisms may contribute to this outcome, but habitat fragmentation is generally considered the main external driver of local species extinction. This phenomenon may increase ecosystem variability and reduce resilience to other disturbances such as climate change [39]. Joshua et al.’s study on Cenozoic rodent community diversity revealed that climate change may indirectly affect community diversity by altering habitat vegetation characteristics; they found that drought and high temperatures simultaneously exert positive impacts on rodent diversity, which is consistent with the findings of this study that temperature directly had a positive impact on local rodent diversity [40]. Moisture conditions positively affect community diversity through vegetation canopy density, which may be manifested at smaller scales. At the metacommunity scale, moisture directly had a negative impact on its α and β diversity. Seasonal precipitation, temperature, vegetation biomass, and abundance and richness collectively drive the functional and species diversity of small mammal communities in Mexican rainforests [41], further illustrating the diverse impacts of climate change on rodent community diversity.
In summary, the impacts of climatic factors on community diversity are basically similar. However, temperature had a consistent effect on community diversity at both local and metacommunity scales, while moisture had different effects on community diversity at these two scales. The reason for this phenomenon may be that animal and plant communities are more sensitive to moisture than to temperature, leading to asynchronous variation at different scales. Additionally, the unequal response to climatic factors of dominant species that constitute local and metacommunities were also a reason why regional processes differ from local phenomena.
5. Conclusions
The mechanisms by which climatic condition fluctuations affect rodent local communities and metacommunities follow complex pathways. These pathways vary due to the distinct regulatory mechanisms of water and thermal conditions. Specifically, precipitation exerts an indirect positive effect on rodent communities primarily by modifying habitat vegetation characteristics, while temperature imposes a direct positive effect on rodent communities or an indirect positive effect through regulating vegetation traits. Metacommunities are the coupled products of local communities established through species migration and habitat filtering, leading to complex relationships between local communities and regional processes, which are manifested through multiple indicators such as the total individual number and diversity of these communities. When metacommunities remain stable, β-diversity among local communities tends to exhibit variations in response to changes in environmental factors. Anthropogenic disturbances exert a non-negligible impact on environmental factors.
The Alxa Desert ecosystem is a typical fragile ecosystem with extreme imbalance in water and heat. In recent years, due to increasingly severe human disturbances, grasslands have undergone severe degradation and desertification, and rodent infestations have occurred on a large scale. Therefore, understanding the fluctuation patterns of rodent community abundance and diversity, as well as the responses of rodent communities to climatic conditions, helps predict changes in local and metacommunities induced by climate change. This is of great significance for protecting biodiversity in desert ecosystems and providing support for eco-environmental management measures. In future studies, we will further incorporate anthropogenic disturbance as a key explanatory variable to analyze the change mechanisms of rodent communities under the combined effects of anthropogenic disturbance and climatic factors.
Author Contributions
Conceptualization, R.Z. and S.Y. (Suwen Yang); methodology, R.Z. and S.Y. (Suwen Yang); investigation, R.Z., S.Y. (Suwen Yang), X.L., Y.J. and L.L.; data curation, R.Z., S.Y. (Suwen Yang), X.L., Y.J. and L.L.; writing—original draft preparation, R.Z.; writing—review and editing, X.W., S.Y. (Shuai Yuan) and H.F.; project administration, X.W.; funding acquisition, X.W., S.Y. (Shuai Yuan) and H.F. All authors have read and agreed to the published version of the manuscript.
Funding
This research was supported by First Class Discipline Research Special Project of Inner Mongolia Autonomous Region Department of Education (YLXKZX-NND-005; YLXKZX-NND-031), Science and Technology Fundamental Resources Investigation Programme (2023FY100305), Basic Scientific Research Business Expenses of Universities Directly under Inner Mongolia Autonomous Region (BR220106, BR221307, BR221037), Inner Mongolia Natural Science Foundation (2023MS03025), Grassland Ecological Protection and Restoration Treatment Subsidy (Z75070050001-2110405), The 2022 Inner Mongolia Autonomous Region Youth Science and Technology Talent Development Plan (NJYT22044), and Inner Mongolia Agricultural University Major Projects (RZ1900001196).
Institutional Review Board Statement
Ethical review and approval were waived for this study due to the fact that the research only involved non-invasive field observations of wild rodent populations, without any capture, handling, or manipulation of the animals. All field surveys were conducted in compliance with the national wildlife protection regulations of the People’s Republic of China.
Data Availability Statement
The data used in the experiment has been presented in the corresponding positions in the text. The data used for constructing the structural equation model has been uploaded to FigShare at https://doi.org/10.6084/m9.figshare.30646592 (accessed on 21 December 2025).
Acknowledgments
We would like to thank the graduate students at the Rodent Research Center of the College of Grassland Science, Inner Mongolia Agricultural University, for their assistance during the field data collection period.
Conflicts of Interest
The funders had no role in the design of the study; in the collection, analyses, or interpretation of data; in the writing of the manuscript; or in the decision to publish the results.
Abbreviations
The following abbreviations are used in this manuscript:
| βSIM | Spatial Species Turnover Index |
| βSNE | Nestedness of Assemblages Index |
| βSOR | Sørensen Pairwise Dissimilarity |
| SEM | Structural Equation Model |
| NNFI | Non-Normed Fit Index |
| CFI | Comparative Fit Index |
References
- Flowerdew, J.R.; Shore, R.F.; Poulton, S.M.C.; Sparks, T.H. Live trapping to monitor small mammals in Britain. Mammal Rev. 2010, 34, 31–50. [Google Scholar] [CrossRef] [Scilit]
- Leis, S.A.; Leslie, D.M.; Engle, D.M.; Fehmi, J.S. Small mammals as indicators of short-term and long-term disturbance in mixed prairie. Environ. Monit. Assess. 2008, 137, 75. [Google Scholar] [CrossRef] [Scilit]
- Bueno, C.; Ruckstuhl, K.E.; Arrigo, N.; Aivaz, A.N.; Neuhaus, P. Impacts of cattle grazing on small-rodent communities: An experimental case study. Rev. Can. Zool. 2012, 90, 22–30. [Google Scholar] [CrossRef] [Scilit]
- Chase, J.M.; Leibold, M.A. Ecological Niches: Linking Classical and Contemporary Approaches. Austral Ecol. 2004, 29, 602–603. [Google Scholar] [CrossRef] [Scilit]
- Gilpin, M. Single-species metapopulation dynamics: Concepts, models and observations. Metapopul. Dyn. Empir. Theor. Investig. 1991, 42, 17–38. [Google Scholar] [CrossRef] [Scilit]
- Leibold, M.A.; Holyoak, M.; Mouquet, N.; Amarasekare, P.; Chase, J.M.; Hoopes, M.F.; Holt, R.D.; Shurin, J.B.; Law, R.; Tilman, D. The metacommunity concept: A framework for multi-scale community ecology. Ecol. Lett. 2004, 7, 601–613. [Google Scholar] [CrossRef] [Scilit]
- Thomas, H.; Elisabeth, B.-K.; Olena, B.; Florian, B.; Andrea, F.; Michael, G.; Gertrud, H.; Johannes, K.; Paul, M.B.; Jakob, N.; et al. How can the meta-ecosystem approach improve the management of large river networks? In Proceedings of the 44th Conference of International Danube Research, Krems, Austria, 6–9 February 2023; pp. 1–6. [Google Scholar]
- Eccard, J.; Ferreira, C.M.; Arce, A.P.; Dammhahn, M. Top-down effects of foraging decisions on local, landscape and regional biodiversity of resources (DivGUD). Ecol. Lett. 2022, 25, 3–16. [Google Scholar] [CrossRef] [Scilit]
- Cha, M.; Wu, X.; Fu, H.; Yuan, S.; Zhang, X. An empirical research of rodent metacommunities in Alashan Desert. Acta Ecol. Sin. 2015, 35, 5612–5622. [Google Scholar] [CrossRef] [Scilit]
- Zhang, X.; Wu, X.; Fu, H.; Yuan, S.; Cha, M. The Mongolian Gerbils Meta-population in Habitat Fragmentation in Alxa Desert: A Field Verification Study. Chin. J. Zool. 2013, 48, 834–843. [Google Scholar]
- Vanschoenwinkel, B.; Vries, C.D.; Seaman, M.; Brendonck, L. The role of metacommunity processes in shaping invertebrate rock pool communities along a dispersal gradient. Oikos 2010, 116, 1255–1266. [Google Scholar] [CrossRef]
- Myers, P.; Lundrigan, B.L.; Hoffman, S.M.G.; Haraminac, A.P.; Seto, S.H. Climate-induced changes in the small mammal communities of the Northern Great Lakes Region. Glob. Change Biol. 2010, 15, 1434–1454. [Google Scholar] [CrossRef] [Scilit]
- Jarema, S.I.; Samson, J.; Mcgill, B.J.; Humphries, M.M. Variation in abundance across a species’ range predicts climate change responses in the range interior will exceed those at the edge: A case study with North American beaver. Glob. Change Biol. 2010, 15, 508–522. [Google Scholar] [CrossRef] [Scilit]
- Temperli, C.; Bugmann, H.; Elkin, C. Cross-scale interactions among bark beetles, climate change, and wind disturbances: A landscape modeling approach. Ecol. Monogr. 2013, 83, 383–402. [Google Scholar] [CrossRef] [Scilit]
- Khishigbayar, J.; Fernández-Giménez, M.E.; Angerer, J.P.; Reid, R.S.; Chantsallkham, J.; Baasandorj, Y.; Zumberelmaa, D. Mongolian rangelands at a tipping point? Biomass and cover are stable but composition shifts and richness declines after 20 years of grazing and increasing temperatures. J. Arid Environ. 2015, 115, 100–112. [Google Scholar] [CrossRef] [Scilit]
- Rebelo, H.; Tarroso, P.; Jones, G. Predicted impact of climate change on European bats in relation to their biogeographic patterns. Glob. Change Biol. 2010, 16, 561–576. [Google Scholar] [CrossRef] [Scilit]
- Loarie, S.R.; Duffy, P.B.; Hamilton, H.; Asner, G.P.; Field, C.B.; Ackerly, D.D. The velocity of climate change. Nature 2009, 462, 1052–1055. [Google Scholar] [CrossRef] [Scilit]
- Garroway, C.J.; Bowman, J.; Cascaden, T.J.; Holloway, G.L.; Mahan, C.G.; Malcolm, J.R.; Steele, M.A.; Turner, G.; Wilson, P.J. Climate change induced hybridization in flying squirrels. Glob. Change Biol. 2010, 16, 113–121. [Google Scholar] [CrossRef] [Scilit]
- Morris, C.; Badik, K.J.; Morris, L.R.; Weltz, M.A. Integrating precipitation, grazing, past effects and interactions in long-term vegetation change. J. Arid Environ. 2016, 124, 111–117. [Google Scholar] [CrossRef] [Scilit]
- Isbell, F.; Craven, D.; Connolly, J.; Loreau, M.; Schmid, B.; Beierkuhnlein, C.; Bezemer, T.M.; Bonin, C.; Bruelheide, H.; Luca, E.D. Biodiversity increases the resistance of ecosystem productivity to climate extremes. Nature 2015, 526, 574–577. [Google Scholar] [CrossRef] [Scilit]
- Zhang, F.; Fu, H.; Wu, X.; Yang, Z.; Zhang, X. Spatial synchrony in population dynamics of desert rodents. Acta Theriol. Sin. 2011, 31, 211–218. [Google Scholar] [CrossRef]
- Yuan, S.; Wu, X.; Fu, H.; Yang, Z.; Zhang, X. Multi-scales analysis on diversity of desert rodent communities under different disturbances. Acta Ecol. Sin. 2011, 31, 1982–1992. [Google Scholar] [CrossRef]
- Tim, N. Future effects of climate and land-use change on terrestrial vertebrate community diversity under different scenarios. Proc. R. Soc. B Biol. Sci. 2018, 285, 20180792. [Google Scholar] [CrossRef] [Scilit]
- Brodie, J.F. Synergistic effects of climate change and agricultural land use on mammals. Front. Ecol. Environ. 2016, 14, 20–26. [Google Scholar] [CrossRef] [Scilit]
- Kamár, P. Principles and Practice of Structural Equation Modeling, 5th ed.; Individual & Society/Clovek a Spolocnost: Kosice, Slovakia, 2024; Volume 27. [Google Scholar] [CrossRef] [Scilit]
- Selonen, V.; Helle, S.; Laaksonen, T.; Ahola, M.P.; Lehikoinen, E.; Eeva, T. Identifying the paths of climate effects on population dynamics: Dynamic and multilevel structural equation model around the annual cycle. Oecologia 2021, 195, 525–538. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yaworsky, P.M.; Hussain, S.T.; Riede, F. Climate-driven habitat shifts of high-ranked prey species structure Late Upper Paleolithic hunting. Sci. Rep. 2023, 13, 4238. [Google Scholar] [CrossRef] [Scilit]
- Franco, A.L.C.; Adams, B.J.; Diaz, M.A.; Lemoine, N.P.; Dragone, N.B.; Fierer, N.; Lyons, W.B.; Hogg, I.; Wall, D.H. Response of Antarctic soil fauna to climate-driven changes since the Last Glacial Maximum. Glob. Change Biol. 2022, 28, 644–653. [Google Scholar] [CrossRef] [Scilit]
- Levin, S.A. Dispersion and population interactions. Am. Nat. 1974, 108, 207–228. [Google Scholar] [CrossRef] [Scilit]
- Lawton, J.H. Are there general laws in ecology? OIKOS 1999, 84, 177–192. [Google Scholar] [CrossRef] [Scilit]
- Riddell, E.A.; Iknayan, K.J.; Hargrove, L.; Tremor, S.; Patton, J.L.; Ramirez, R.; Wolf, B.O.; Beissinger, S.R. Exposure to climate change drives stability or collapse of desert mammal and bird communities. Science 2021, 371, 633–636. [Google Scholar] [CrossRef] [Scilit]
- Heisler, L.M.; Somers, C.M.; Poulinheisler, R.G. Rodent populations on the northern Great Plains respond to weather variation at a landscape scale. J. Mammal. 2014, 90, 82–90. [Google Scholar] [CrossRef] [Scilit]
- Wu, X.D.; A, J.; Fu, H.P.; Heng, J. Dynamic characteristics of desert rodent community patterns under different anthropogenic disturbances-Canonical correlation analysis of animal and plant communities. J. Ecol. 2008, 28, 5999–6017. [Google Scholar] [CrossRef]
- Frank, D.; Reichstein, M.; Bahn, M.; Thonicke, K.; Frank, D.; Mahecha, M.D.; Smith, P.; Velde, M.; Vicca, S.; Babst, F. Effects of climate extremes on the terrestrial carbon cycle: Concepts, processes and potential future impacts. Glob. Change Biol. 2015, 21, 2861–2880. [Google Scholar] [CrossRef] [Scilit]
- Wu, J. Progress in the Study of the Impact of Climate Change on Land Biodiversity. Chin. Eng. Sci. 2008, 10, 60–68. [Google Scholar]
- Loreau, M.; Naeem, S.; Inchausti, P.; Wardle, D. Biodiversity and Ecosystem Functioning: Current Knowledge and Future Challenges. Science 2001, 294, 804–808. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tilman, D.; Reich, P.B.; Knops, J.M.H. Biodiversity and ecosystem stability in a decade-long grassland experiment. Nature 2006, 441, 629–632. [Google Scholar] [CrossRef] [Scilit]
- Santoro, S.; Suarez, C.S.; Rouco, C.; Moreno, S. Long-term data from a small mammal community reveal loss of diversity and potential effects of local climate change. Curr. Zool. 2017, 63, 515–523. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Foley, J.A. Global Consequences of Land Use. Science 2005, 309, 570–574. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Joshua, S.X.; Samantha, H.S.B. The impacts of Cenozoic climate and habitat changes on small mammal diversity of North America. Glob. Planet. Change 2017, 149, 36–52. [Google Scholar] [CrossRef] [Scilit]
- David, M.R.E.; Farías, A.A.; Gerardo, C.; Bi-Song, Y. Two decades of climate driving the dynamics of functional and taxonomic diversity of a tropical small mammal community in western Mexico. PLoS ONE 2017, 12, e0189104. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2025 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.