Article

Overexploitation of the Atlantic Sharpnose Shark (Rhizoprionodon terraenovae) in Marine Priority Regions of Tamaulipas, Mexico: Implications for Wetland Conservation and Data-Limited Fisheries Management


by
Jorge Homero Rodríguez-Castro
1,*,
Sandra Edith Olmeda-de la Fuente
1,*,
Jorge Alejandro Rodríguez-Olmeda
1,
Ulises de Jesús Balderas-Mancilla
2,
Juventino Tovar-Ortíz
1,
Jose Antonio Rangel-Lucio
1 and
Luis Antonio Vázquez-Ochoa
1
1
División de Estudios de Posgrado e Investigación, Instituto Tecnológico de Ciudad Victoria, Tecnológico Nacional de México, Boulevard Emilio Portes Gil No. 1301, Ciudad Victoria 87010, Tamaulipas, Mexico
2
Instituto Tecnológico de Altamira, Tecnológico Nacional de Mèxico, Carretera Tampico-Mante, Km 24.5, Altamira 89600, Tamaulipas, Mexico
*
Authors to whom correspondence should be addressed.
Fishes 2026, 11(5), 268; https://doi.org/10.3390/fishes11050268
Submission received: 25 February 2026 / Revised: 28 March 2026 / Accepted: 23 April 2026 / Published: 30 April 2026
(This article belongs to the Special Issue Ecology of Fish: Age, Growth, Reproduction and Feeding Habits)

Abstract

Artisanal fisheries in Mexico frequently operate with limited data, lacking historical catch and effort series. In this context, the population status of the dogfish (Rhizoprionodon terraenovae) was evaluated for the first time in Priority Marine Regions 45–46 and the area of influence of the Wetland of International Importance Playa Tortuguera Rancho Nuevo, Tamaulipas, using methods based on size frequencies. Between November 2018 and February 2020, 541 artisanal fishing organisms were analyzed in La Barra del Tordo using FISAT II. The von Bertalanffy growth parameters for combined sexes were: L∞ = 105 cm, k = 0.59 years−1, t0 = −0.195 years. Total (Z), natural (M) and fishing (F) mortalities were 4.13, 0.467 and 3.22 years−1, respectively. The average exploitation rate (E = F/Z) was 0.78 (95% CI: 0.745–0.805), exceeding the reference point of 0.5 indicating severe overexploitation. The parameters showed biological consistency (Ø′ = 3.81; M/k = 0.79), and natural mortality was within the range reported for the species. This finding, in a priority region for conservation under the regime of the Conservation Sector of the Marine Ecological Management Program, shows the urgent need to implement fisheries management with an ecosystem approach that guarantees the sustainability of the fishery and the integrity of the coastal ecosystem. The study demonstrates that, even with limited data, it is possible to obtain robust estimates to inform management decisions in natural protected areas
Key Contribution: First quantitative assessment of Rhizoprionodon terraenovae in Tamaulipas priority conservation areas revealing severe overexploitation (E = 0.78) through data-limited methods, highlighting the urgent need for ecosystem-based management to ensure fishery sustainability and coastal ecosystem integrity, with implications for the conservation of associated species such as the Kemp’s ridley sea turtle.

1. Introduction

Small-scale artisanal fisheries constitute the livelihood of millions of people in coastal communities of developing countries [1,2,3,4]. However, these fisheries typically operate under data-limited conditions (“data-poor fisheries”), characterized by the absence of historical catch and effort time series, the lack of species-specific stock assessments, and the scarcity of basic biological information [5,6,7,8,9,10]. This limitation represents one of the most significant challenges for the assessment and sustainable management of fishery resources globally, particularly in high-priority conservation regions [10]. In this context, the relative ease of collecting catch size composition data has driven a rapid global adoption of length-based assessment methods, enabling, for the first time, the preliminary evaluation of numerous fisheries that were previously considered unassessable due to lack of data [11,12].
Coastal sharks of the family Carcharhinidae are fundamental components of tropical and subtropical marine ecosystems, where they act as mid-to-high trophic level predators and contribute to the regulation of food webs [13,14].
Within this group, the Atlantic sharpnose shark (Rhizoprionodon terraenovae) (Richardson, 1837) is a small-sized shark (<150 cm) traditionally considered of “high biological productivity” due to its relatively fast growth rates, early maturity (3–4 years), and high reproductive potential [15,16]. Nevertheless, this perception of resilience has been challenged by evidence of overexploitation in various regions of the Gulf of Mexico [17,18], generating a debate on the actual vulnerability of species with “fast” life histories facing intense, unregulated fishing pressures [19,20]. However, this resilience is not uniform. Studies in the northern Gulf of Mexico show that the fecundity of R. terraenovae varies spatially, with significantly larger litters west of 88° W. This difference, associated with a greater abundance of prey such as Micropogonias undulatus, suggests that reproductive potential in the western region may be twice that of the eastern region, underscoring the importance of considering such disparities in the assessment and management of its populations [21].
Recently, Wakida-Kusunoki et al. [22] documented the unusual presence of R. terraenovae neonates in a coastal lagoon in the southeastern Gulf of Mexico (Celestún, Yucatán), suggesting that coastal lagoons may function as nursery habitats for the species. In the northern Gulf of Mexico, however, knowledge of the use of these habitats is scarce, and there are no previous records of neonates in the coastal lagoons of Tamaulipas.
The southern coast of Tamaulipas hosts two Marine Priority Regions for conservation in Mexico: Region 45 “La Pesca-Rancho Nuevo” and Region 46 “Laguna de San Andrés”, designated in the Gulf of Mexico and Caribbean Sea Marine and Regional Ecological Zoning Program [23]. These regions belong to the Conservation Sector, whose objective is “the promotion of protection, restoration, and conservation of ecosystems, natural resources, environmental goods and services, aimed at fostering their use while guaranteeing sustainable development” [23]. Additionally, the Playa Tortuguera Rancho Nuevo site has been designated as a Wetland of International Importance (Ramsar Site No. 1326) due to its critical role in the nesting of the Kemp’s ridley sea turtle (Lepidochelys kempii), an endemic species of the Gulf of Mexico and critically endangered [24,25].
In these Marine Priority Regions, intense artisanal fishing activity targets multiple species, including R. terraenovae, which is caught both in directed longline fisheries and as bycatch in scale fish fisheries [23,26]. A crucial aspect, scarcely addressed in the literature, is the role of R. terraenovae as a natural predator of sea turtle neonates [27], as occurs with other shark species such as the blacktip reef shark (Carcharhinus melanopterus) [28] and in other regions such as Malaysia [29] in the predation of sea turtle neonates.
The Management Program of the Playa Rancho Nuevo Sanctuary [26] explicitly recognizes that species such as the sharpnose shark exert predation pressure on neonates during the hatching season (August–November), when they emerge from nests and head to the sea facing high mortality [27], as occurs with other shark species such as the blacktip reef shark (Carcharhinus melanopterus) [28] and in other regions such as Malaysia [29].
Assessing the population status of R. terraenovae in this context becomes relevant not only for fisheries management but also for the conservation of L. kempii. However, controversies persist regarding the true status of the species’ populations in the Gulf of Mexico, with exploitation rate estimates ranging from 0.14 in Campeche [30] to 0.77 in the same region [17], suggesting a complex spatio-temporal dynamic that could be due to methodological differences, regional variations in fishing pressure, or the existence of multiple fishery stocks [31,32,33,34,35].
The hypotheses guiding this study were: (H1) the population of R. terraenovae in Marine Priority Regions 45–46 is overexploited as a result of artisanal fishing pressure; (H2) the overexploitation of this predator has potential implications for the structure of the coastal ecosystem and for the fulfillment of the Conservation Sector objectives; and (H3) despite the limitations inherent to a data-limited fishery, it is possible to obtain robust estimates of population parameters using length–frequency-based methods.
The main objective of this study was to estimate growth and mortality parameters, and to determine the exploitation rate of R. terraenovae in Marine Priority Regions 45–46 and the influence area of the Playa Tortuguera Rancho Nuevo Wetland of International Importance, to assess its population status and analyze the implications of its exploitation for sea turtle conservation and fisheries management in a data-limited context. Our results reveal severe overexploitation (E = 0.78), evidencing the urgent need to implement ecosystem-based management in this priority region.

2. Materials and Methods

2.1. Study Area

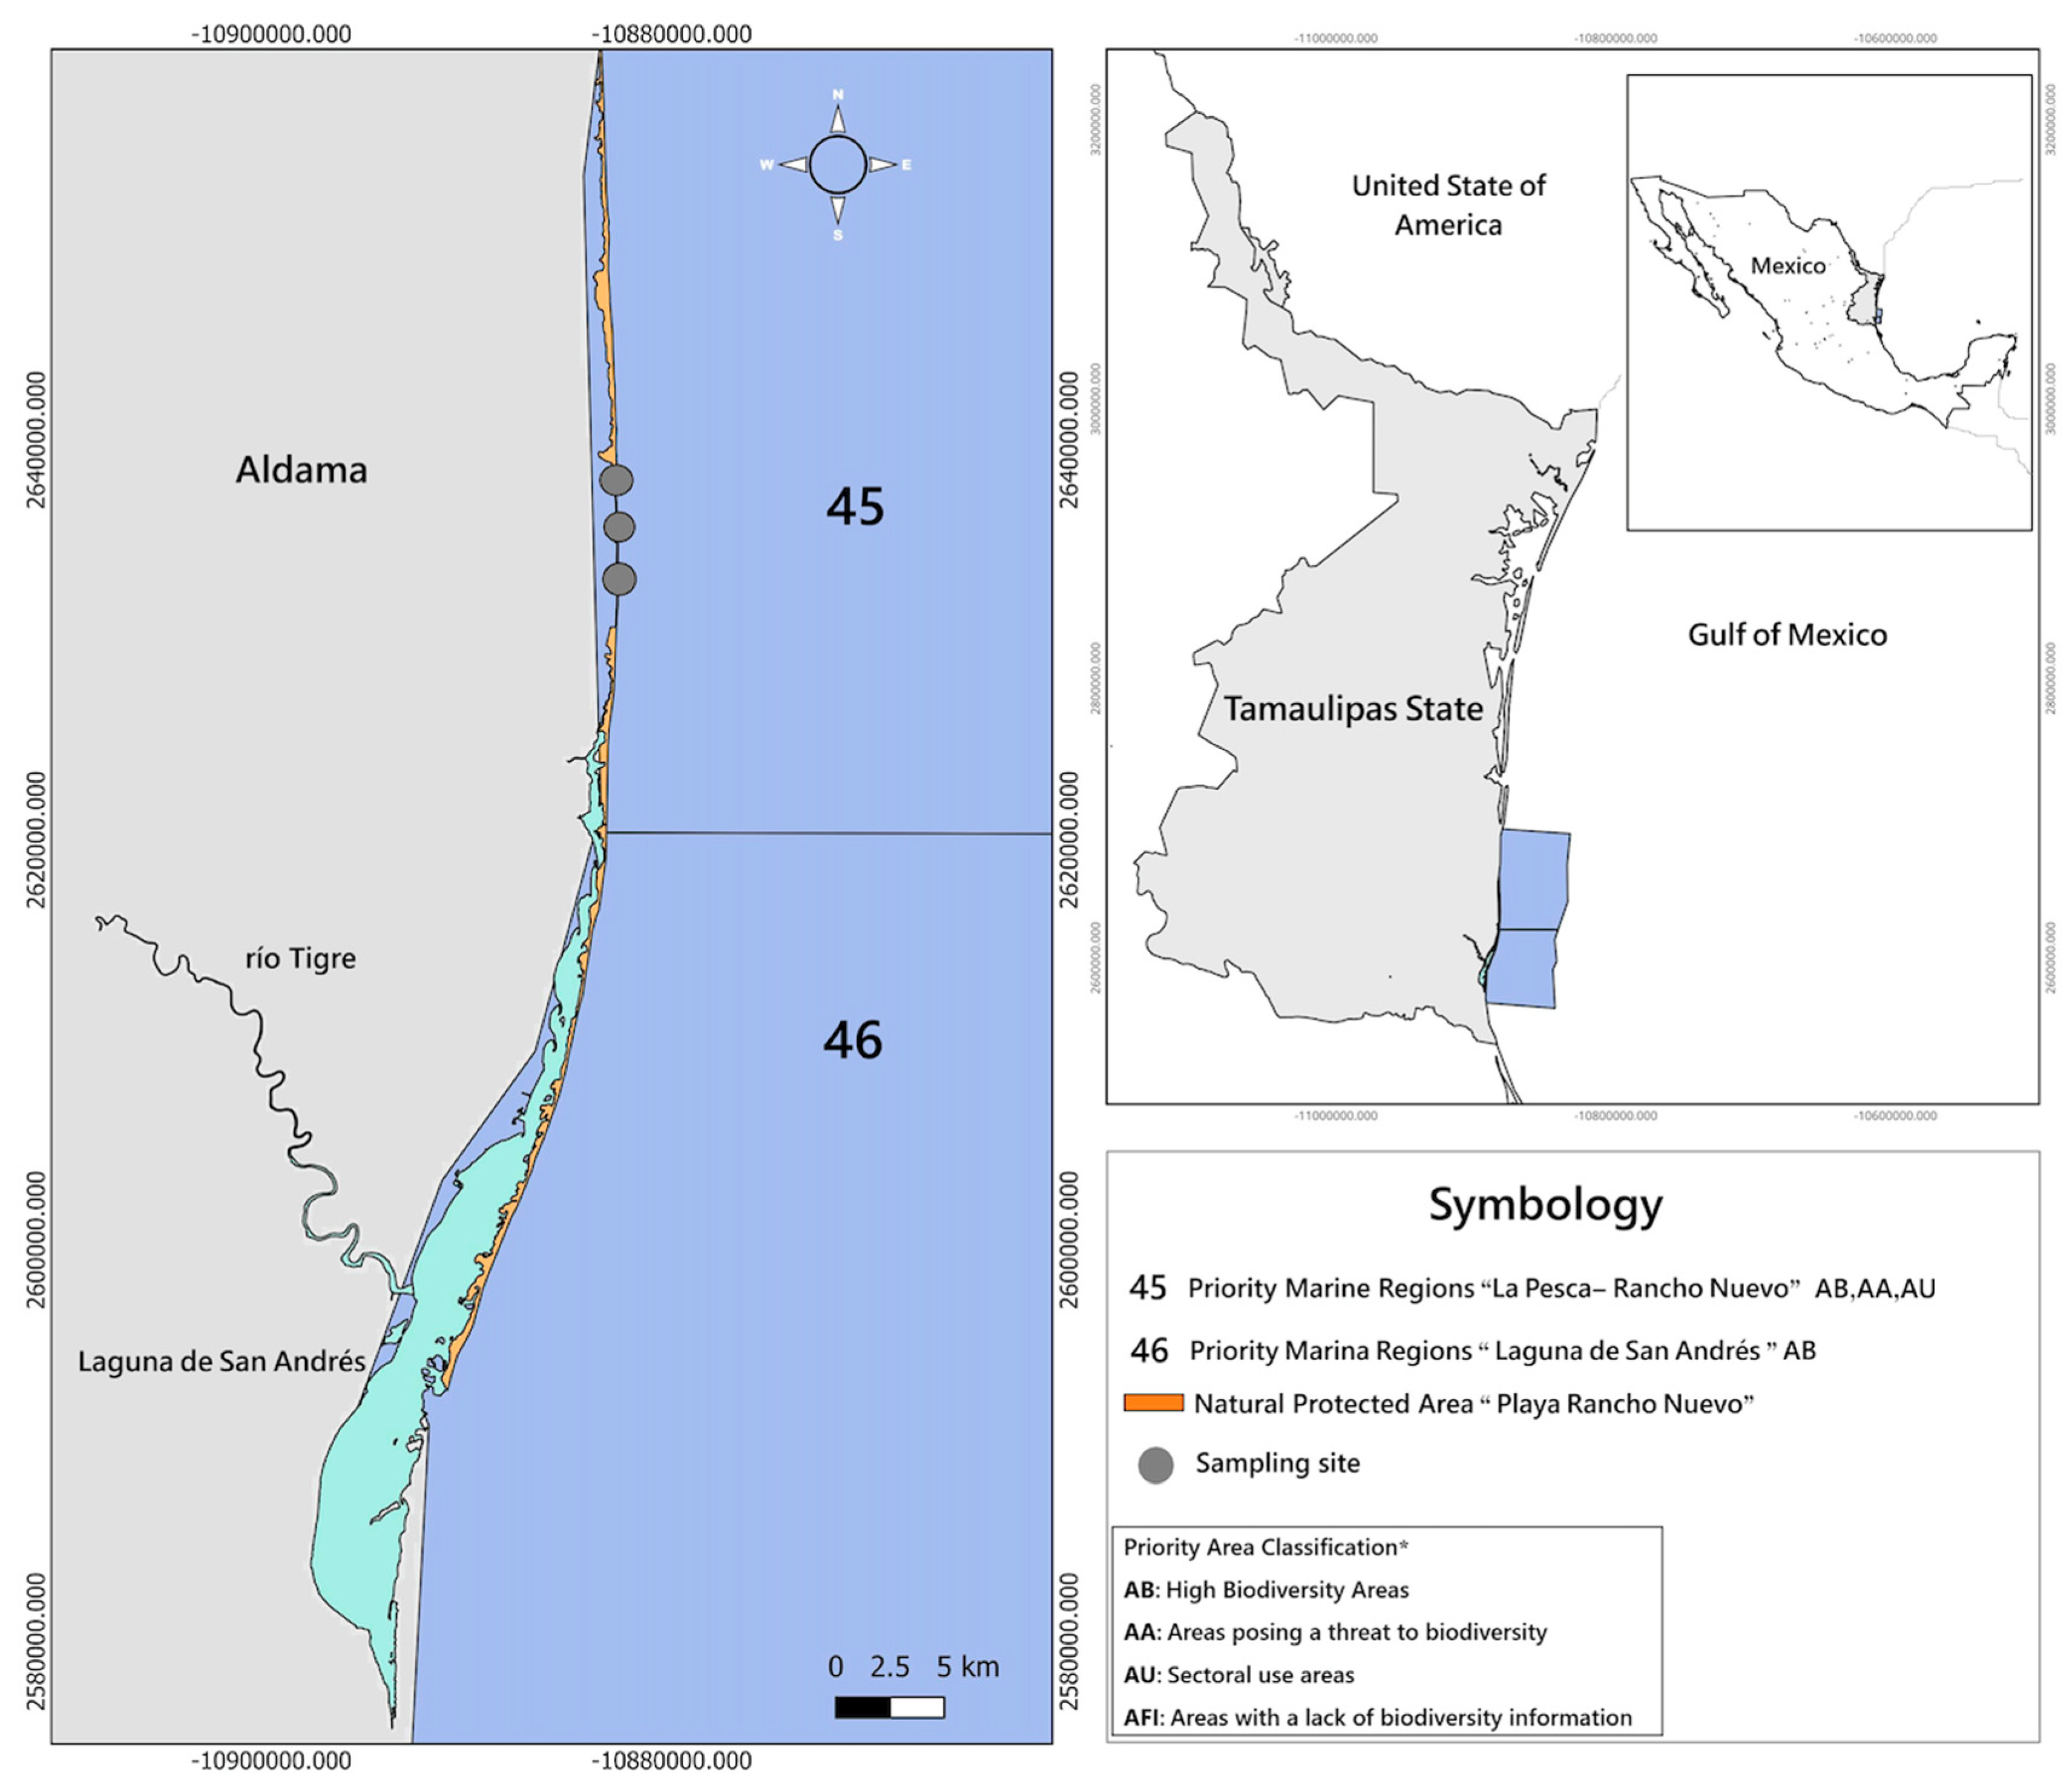
The study was carried out in the town of La Barra del Tordo, municipality of Aldama, Tamaulipas, Mexico (23°03′ N, 97°46′ W), located in the area that includes two Priority Marine Regions for conservation in Mexico: Region 45 “La Pesca-Rancho Nuevo” and Region 46 “Laguna de San Andrés” [36]. and within the area of influence of the Playa Tortuguera Rancho Nuevo Wetland of International Importance (Ramsar Site No. 1326) [24] (Figure 1).
Marine Priority Region 45 “La Pesca-Rancho Nuevo” is located between 23°30′ and 22°54′ north latitude and 97°48′36″ and 97°18′36″ west longitude, with an area of 2955 km2 [26]. This region is characterized by a warm semi-arid climate with rainfall in summer, an average annual temperature of 22–26 °C, and the occurrence of tropical storms, hurricanes and hurricanes. Geologically, it has sedimentary rocks, a slope with a gentle slope and a wide platform. It includes coastal lagoons, beaches, coastal dunes, marshes and estuaries. Biodiversity includes molluscs, polychaetes, echinoderms, crustaceans, fish, turtles, birds, marine mammals and mangroves, with endemism of turtles (L. kempii) and constitutes a nesting and reproduction area for turtles [36,37].
Priority Marine Region 46 “Laguna de San Andrés” is located between 22°54′ and 22°25′48″ north latitude and 97°56′24″ and 97°23′24″ west longitude, with an area of 2384 km2 [36]. It has a temperate subhumid climate, average annual rainfall of 635–791 mm, evaporation of 1475–1876 mm per year, average annual temperature of 17–24 °C, with hurricanes in summer and northern hurricanes in winter. Geologically, it has a coastline of marginal seas with sedimentary rocks and a floodable depression. It includes lagoons, swamps, meadows and beaches, with medium eutrophication. Biodiversity includes molluscs, crustaceans, fish, turtles, birds, seagrasses (Ruppia maritima) and mangroves (white mangrove Avicennia tinctoria and red mangrove Rhizophora mangle), with high ecological integrity in seagrass meadows, dunes and beaches. It is a growing and feeding area for crustaceans and fish, and for the growth of molluscs [36].
The Playa Tortuguera Rancho Nuevo site was designated as a Wetland of International Importance (Ramsar Site No. 1326) on 2 February 2004, with an area of 30 hectares in its main polygon and an area of influence that covers marine areas up to 30 nautical miles [24]. This designation recognizes the critical importance of this site for the nesting of the olive ridley turtle (L. kempii), a species endemic to the Gulf of Mexico and critically endangered.
The Marine and Regional Ecological Management Program for the Gulf of Mexico and the Caribbean Sea [23] classifies these regions within the Conservation Sector, whose objective includes “the promotion of the protection, restoration and conservation of ecosystems, natural resources, environmental goods and services, tending to promote their use while guaranteeing sustainable development.” This instrument recognizes the need to reconcile productive activities, such as artisanal fishing, with conservation objectives.
The sea surface temperature in the region has an annual average of 24 °C, with maximums in summer (29–30 °C) and minimums in winter (18–20 °C) [38]. The nesting season of the olive ridley turtle runs from April to August, with the hatching and emergence season of neonates between August and November [26].
Artisanal and riverine fishing is the main economic activity of La Barra del Tordo and other surrounding communities such as Tepehuajes and Carbonera. Small, outboard-powered fiberglass boats (“pangas”) operate from the shore of the beach to 30 nautical miles, using various fishing gears: gillnets (anchored), bottom longlines (1000–1200 hooks), and handlines for shark fishing [26,39]. The fleet operates year-round, with higher landings in spring–summer. The main target species are trout (Cynoscion nebulosus), red snapper (Lutjanus campechanus), snook, croaker, and several species of small sharks, including R. terraenovae, known locally as “dogfish” [23,26]. According to the characterization of the Priority Marine Regions, low-impact “artisanal fishing (oysters, crabs, scales)” is carried out in this area, although without prior quantitative evaluations [36].

2.2. Biological Sampling

Monthly sampling was conducted during the period from November 2018 to February 2020. The organisms were obtained directly from the landings of artisanal fishing in La Barra del Tordo, with the collaboration of local fishermen. Each specimen was recorded: (1) total length (LT) with an accuracy of 1 mm, measured from the tip of the snout to the end of the caudal fin in a natural position; (2) gutted weight (PE) with an accuracy of 1 g using a Royal Universal digital scale (capacity 10 kg); and (3) sex determined by the presence (male) or absence (female) of gonopterygians.

2.3. Data Analysis

Since this fishery is classified as data-limited, without historical catch and effort series or previous evaluations, analysis methods based exclusively on size frequencies were selected, which have been widely validated for this type of context [40,41].
It is important to note that methods based on size frequencies assume that the sample obtained is representative of the size structure of the exploited population in the study area [40]. While our sampling was systematic over 16 months and covered landings by the local artisanal fleet, we recognize that representativeness may be limited by the selectivity of the fishing gear used (longline and gillnets) and by the spatial distribution of the species. The results should therefore be interpreted as reflecting the status of the portion of the stock accessible to artisanal fisheries in Marine Priority Regions 45–46.

2.3.1. Sex Ratio and Size Structure

The observed sex ratio (females:males) was compared with the expected 1:1 ratio using a Chi-square test (X2) with a significance level of α = 0.05 [42]. A Student’s t-test for independent samples was applied to evaluate significant differences in mean total lengths between sexes [42].

2.3.2. Total Length-Eviscerated Weight Relationship

The relationship between total length (L, cm) and eviscerated weight (P, g) was modeled using the power function P = a·Lb [43], where “a” is the condition factor and “b” is the allometry coefficient. Parameters were estimated by linear regression of logarithmically transformed data: log(P) = log(a) + b·log(L). Growth type was evaluated using a Student’s t-test to determine whether the b value differed significantly from 3 (isometric growth), with H0: b = 3 and Ha: b ≠ 3 [44]. Curves for females and males were compared using the coincident curves analysis proposed by [45].

2.3.3. Growth Parameters

Length growth was modeled using the von Bertalanffy equation [46]: Lt = L∞[1 − exp{−k(t − t0)}]. The parameters L∞ and k were estimated using three length–frequency-based methods included in the FISAT II software package, version 1.2.2. [47]: (1) ELEFAN I routine (Electronic Length Frequency Analysis); (2) Shepherd’s method; and (3) Powell-Wetherall method. These methods are particularly appropriate for data-limited fisheries, as they require only length information and do not depend on chronological age data [48].
The parameter t0 was estimated using Pauly’s empirical equation [48]. To assess uncertainty in L∞ and k estimates, a non-parametric bootstrap procedure [49] was applied with 3000 replicates, using the resampling module of SPSS software (PASW Statistics 18, IBM Corp., Armonk, NY, USA). Medians of bootstrap distributions are reported as point estimates, and the 2.5 and 97.5 percentiles as 95% confidence intervals.
The quality of growth estimates was evaluated using the Phi prime growth performance index (Ø′ = log10k + 2·log10L∞) proposed by Pauly & Munro [50]. This index allows comparison of estimates from this study with those reported in the literature, under the assumption that phylogenetically close species exhibit similar Ø′ values [51].

2.3.4. Total Mortality (Z)

Total mortality (Z, years−1) was estimated using two methods appropriate for data-limited contexts: (1) linearized catch curve [40]; and (2) the Jones and van Zalinge method [52], which is an extension of the catch curve method that uses grouped length–frequency data and does not require complete age conversion.
Since Z estimates are sensitive to the k value used in length-age conversion [50], two k values were employed: that obtained by ELEFAN I (k = 0.59) and that obtained by Shepherd’s method (k = 0.78). This generated four Z estimates: Z1 (catch curve with kELEFAN), Z2 (catch curve with kShepherd), Z3 (Jones-van Zalinge with kELEFAN), and Z4 (Jones-van Zalinge with kShepherd).

2.3.5. Natural Mortality (M)

Natural mortality (M, years−1) was estimated using Pauly’s empirical equation [53] for fish, which relates M to growth parameters and environmental temperature: log10M = −0.0066 − 0.279·log10L∞ + 0.6543·log10k + 0.4634·log10T, where T is the mean annual water temperature (24 °C for the study area) [38]. Two M estimates were obtained using the two k values: M1 (with kELEFAN) and M2 (with kShepherd).

2.3.6. Fishing Mortality (F) and Exploitation Rate (E)

Fishing mortality (F, years−1) was calculated by subtraction: F = Z − M [43]. Using the four Z estimates and the two M estimates, eight F values were generated. The exploitation rate (E) was calculated as E = F/Z [43], obtaining 32 estimates. Following Gulland’s criterion [54], E = 0.5 was considered as the target reference point, where F = M.

2.3.7. Uncertainty Analysis and Selection of Robust Estimates

To identify E estimates with lower uncertainty, the confidence interval length (CIL = upper limit − lower limit) was calculated for each combination. Those with the smallest CIL were selected as the most robust estimates. Two-way ANOVA was applied to evaluate the effect of the factors “Z estimation method” and “F estimation method” on E, and one-way ANOVA to compare estimates with lower variability (α = 0.05).

2.3.8. Declaration on the Use of Artificial Intelligence

During the preparation of this manuscript, no generative artificial intelligence tools were used for the generation of text, data, graphics, or for study design, data collection, analysis, or interpretation of results. Statistical and length–frequency analysis software (SPSS version 18 and the FISAT II package, version 1.2.2.) were used in a conventional manner.

3. Results

3.1. Sample Composition and Population Structure

A total of 541 R. terraenovae organisms caught by artisanal fisheries in Marine Priority Regions 45–46 and the influence area of the Playa Tortuguera Rancho Nuevo Wetland of International Importance, Tamaulipas, Mexico, were analyzed during the period November 2018—February 2020. The sample consisted of 260 females (48.1%) and 281 males (51.9%). The female:male sex ratio (0.93:1) did not differ significantly from the expected 1:1 ratio (X2 = 0.642, df = 1, p = 0.423), indicating sexual balance in the exploited population.
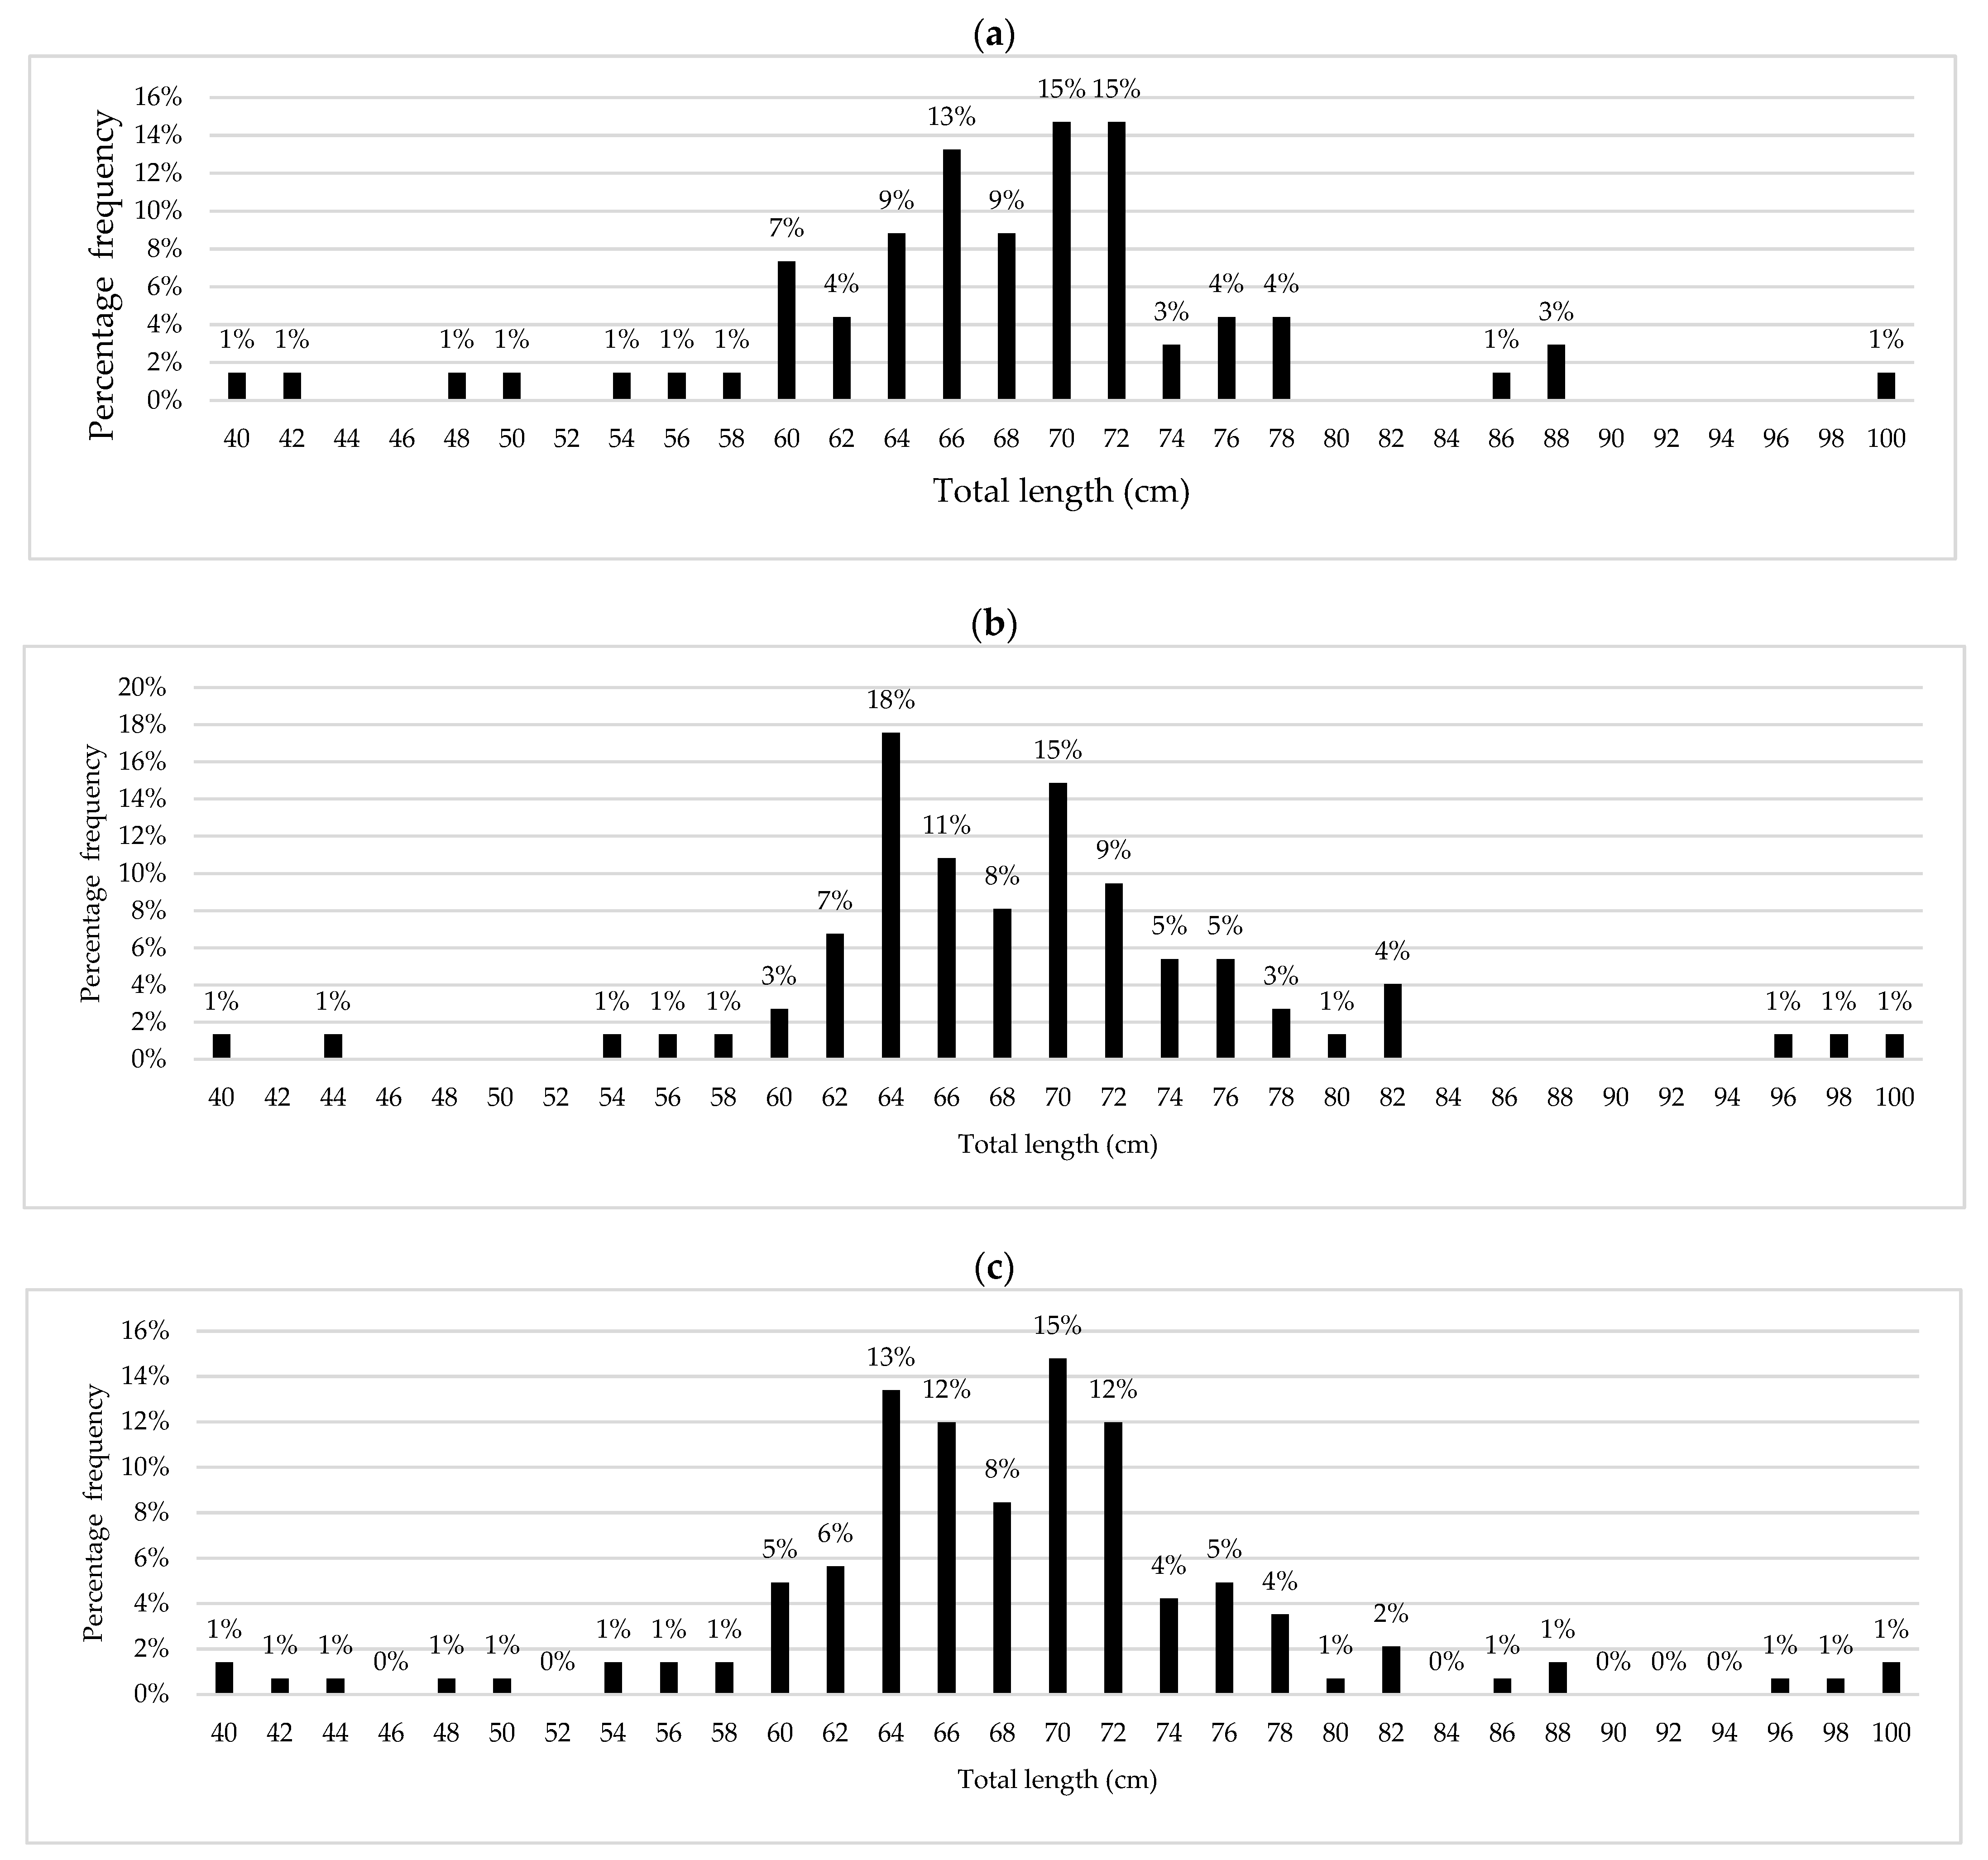
The total length frequency distribution showed a similar unimodal pattern for both sexes (Figure 2). Females exhibited a length range of 40 to 100 cm, with a mean of 66.99 ± 12.3 cm SD and a mode in the 66–68 cm class (Figure 2a). Males showed a slightly smaller range (40–97 cm), with a mean of 66.98 ± 11.9 cm SD and the highest concentration of individuals in the 64–70 cm classes (Figure 2b). For combined sexes (n = 541), the range was 40 to 100 cm with a mean of 66.99 ± 12.1 cm SD, showing a pronounced mode in the 64–68 cm interval, where approximately 25% of individuals were concentrated, with a gradual decrease towards larger (>85 cm) and smaller (<50 cm) sizes (Figure 2c).
No significant differences were found in mean total length between sexes (t = 0.005, df = 539, p = 0.996). Sizes smaller than 50 cm and larger than 85 cm were scarcely represented (<5% of the total), suggesting a low proportion of neonates and long-lived organisms in the catches, with a higher percentage of individuals in juvenile and young adult stages.

3.2. Length–Weight Relationship

Length–weight relationship parameters are presented in Table 1. The b values were close to 3 for both sexes and combined sexes, and the t-test did not reject the isometry hypothesis (p > 0.05). The coincident curves analysis [46] detected no significant differences between sexes (F = −12.39, df = 2537, p < 0.05), justifying the combined analysis.
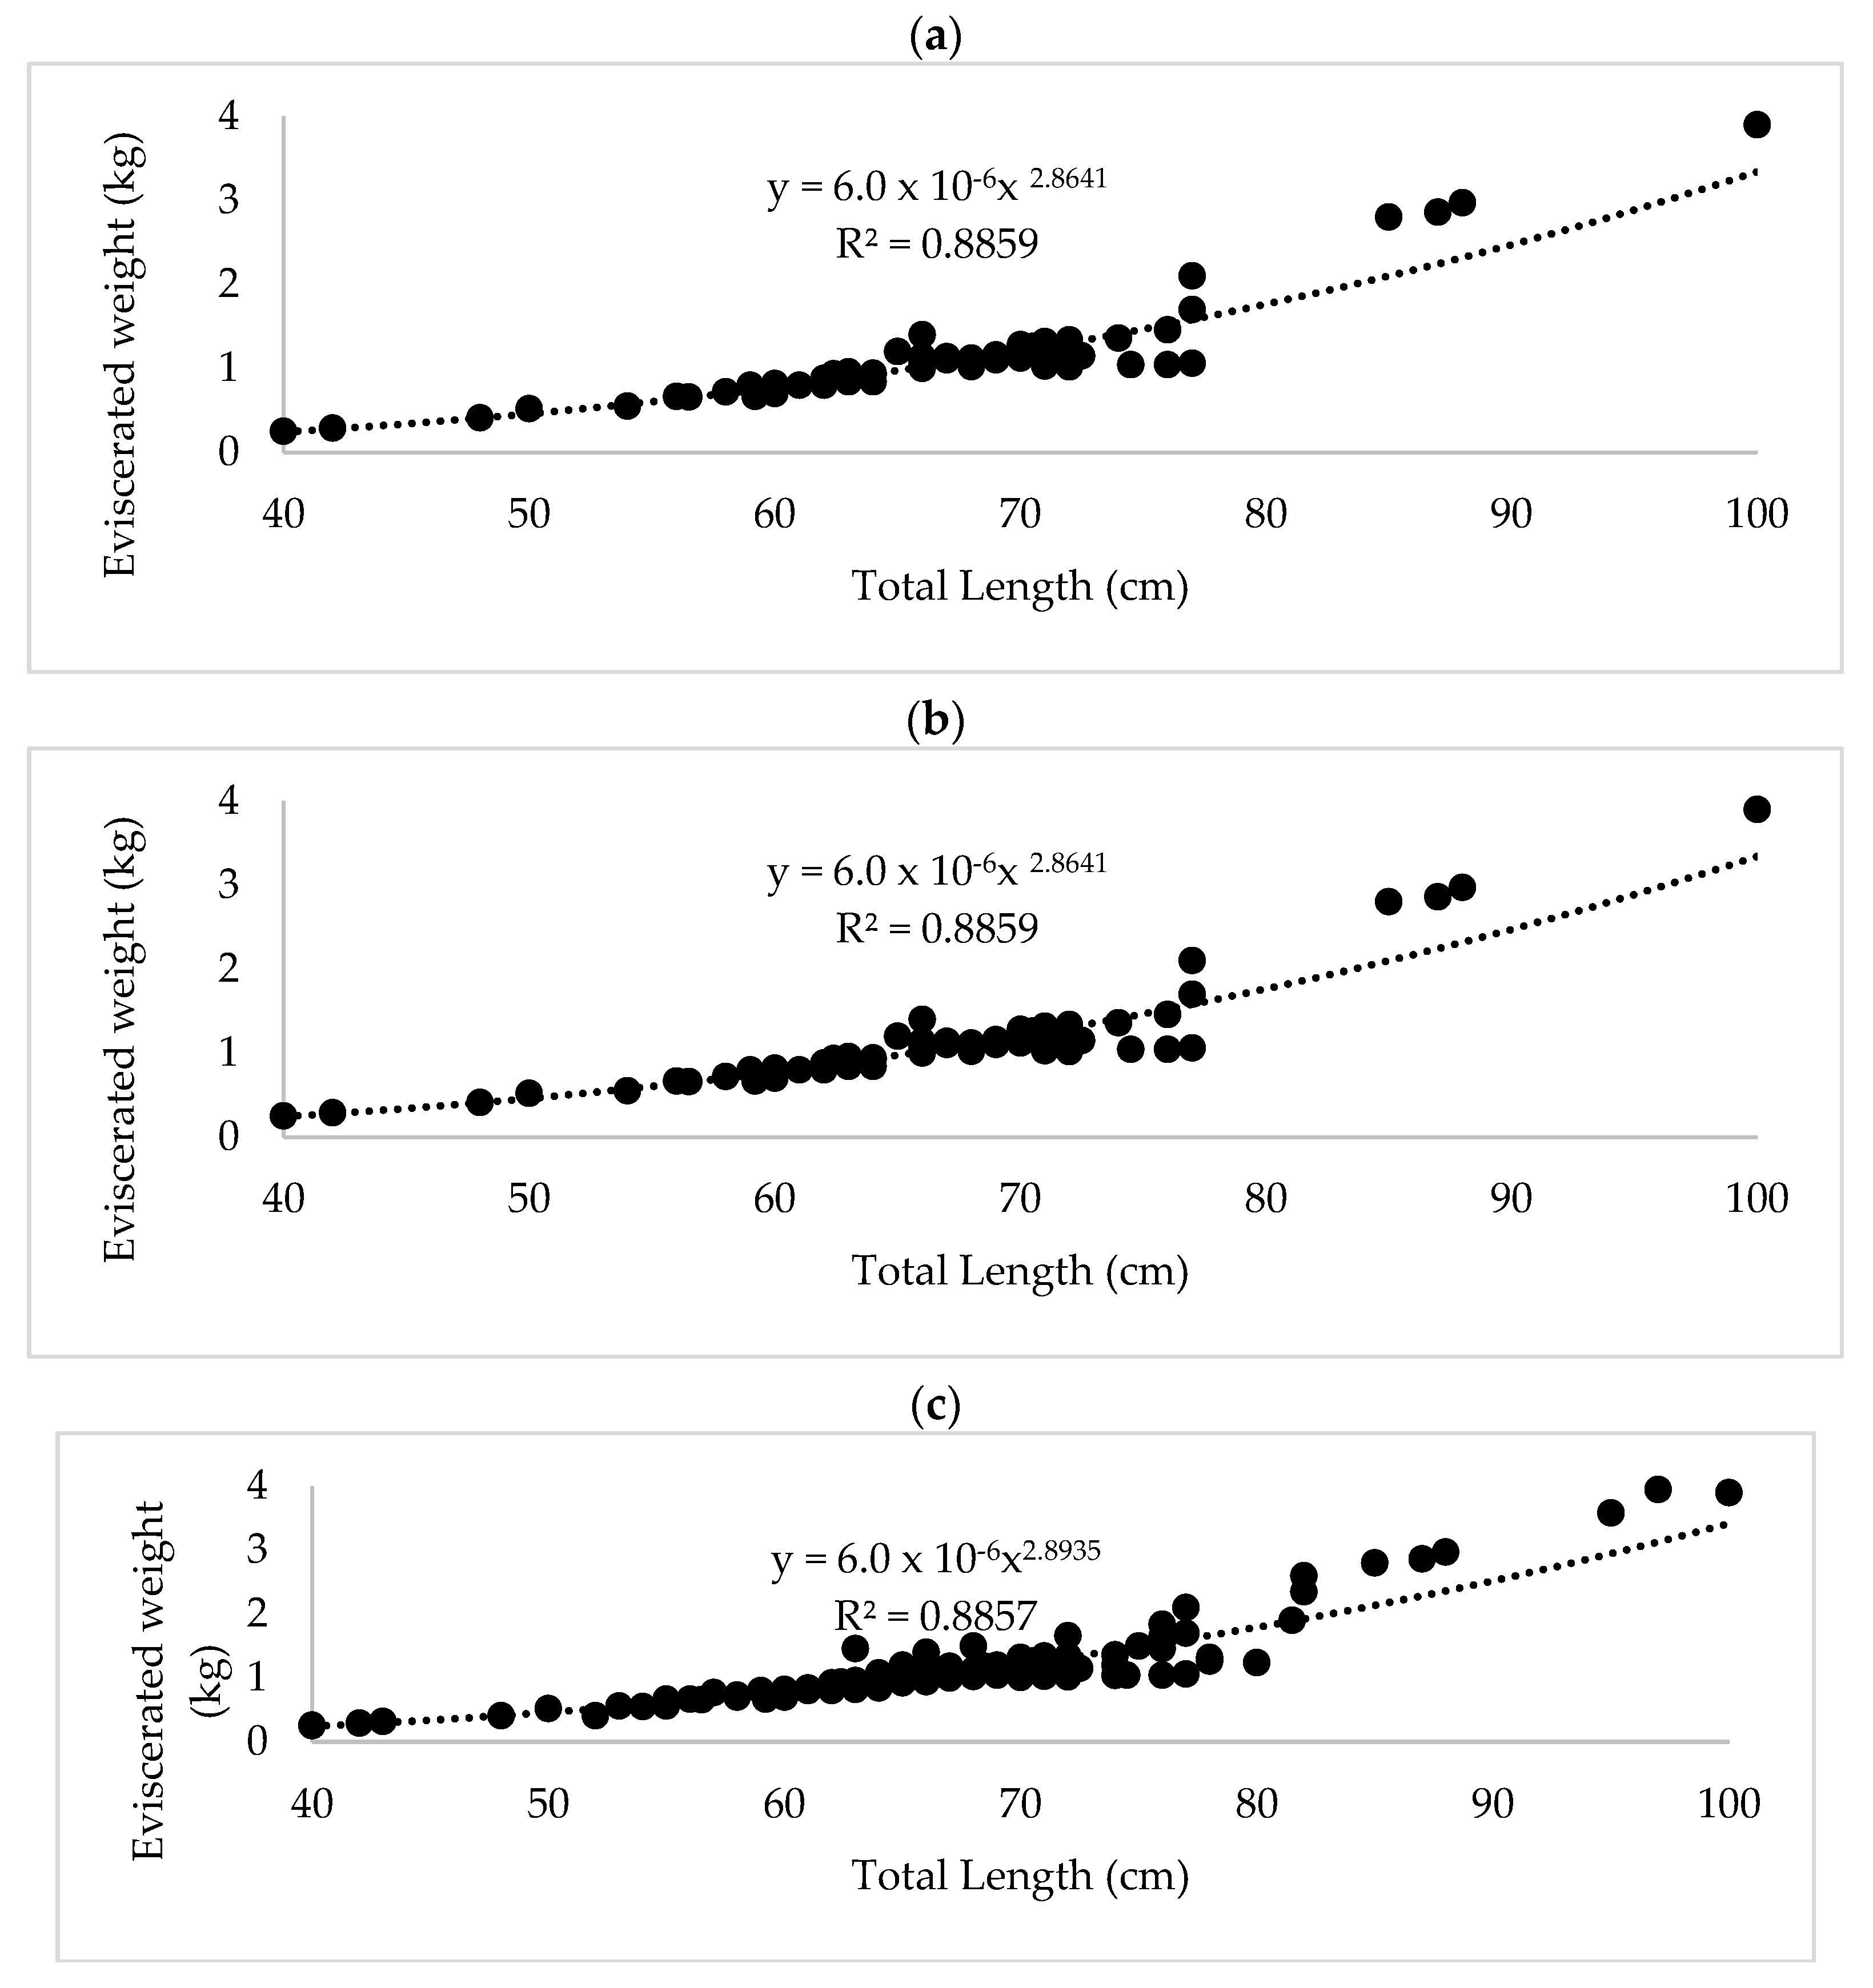
The total length-eviscerated weight relationship for R. terraenovae showed a solid fit to the power model in all analyzed groups (r2 ≥ 0.905; Figure 3). Regression parameters and associated statistical tests are detailed in Table 1. The allometry coefficient (b) values were close to 3 for females (b = 2.86), males (b = 2.92), and combined sexes (b = 2.89). Student’s t-test showed no significant differences from theoretical isometry (p > 0.05 in all cases), confirming isometric growth type for the species in the study area. Likewise, the coincident curves analysis detected no significant differences between sexes (F = −12.39, df = 2537, p < 0.05), which justifies the use of combined analysis to describe the population biometry in Marine Priority Regions 45 and 46 of Tamaulipas.

3.3. Growth Parameters

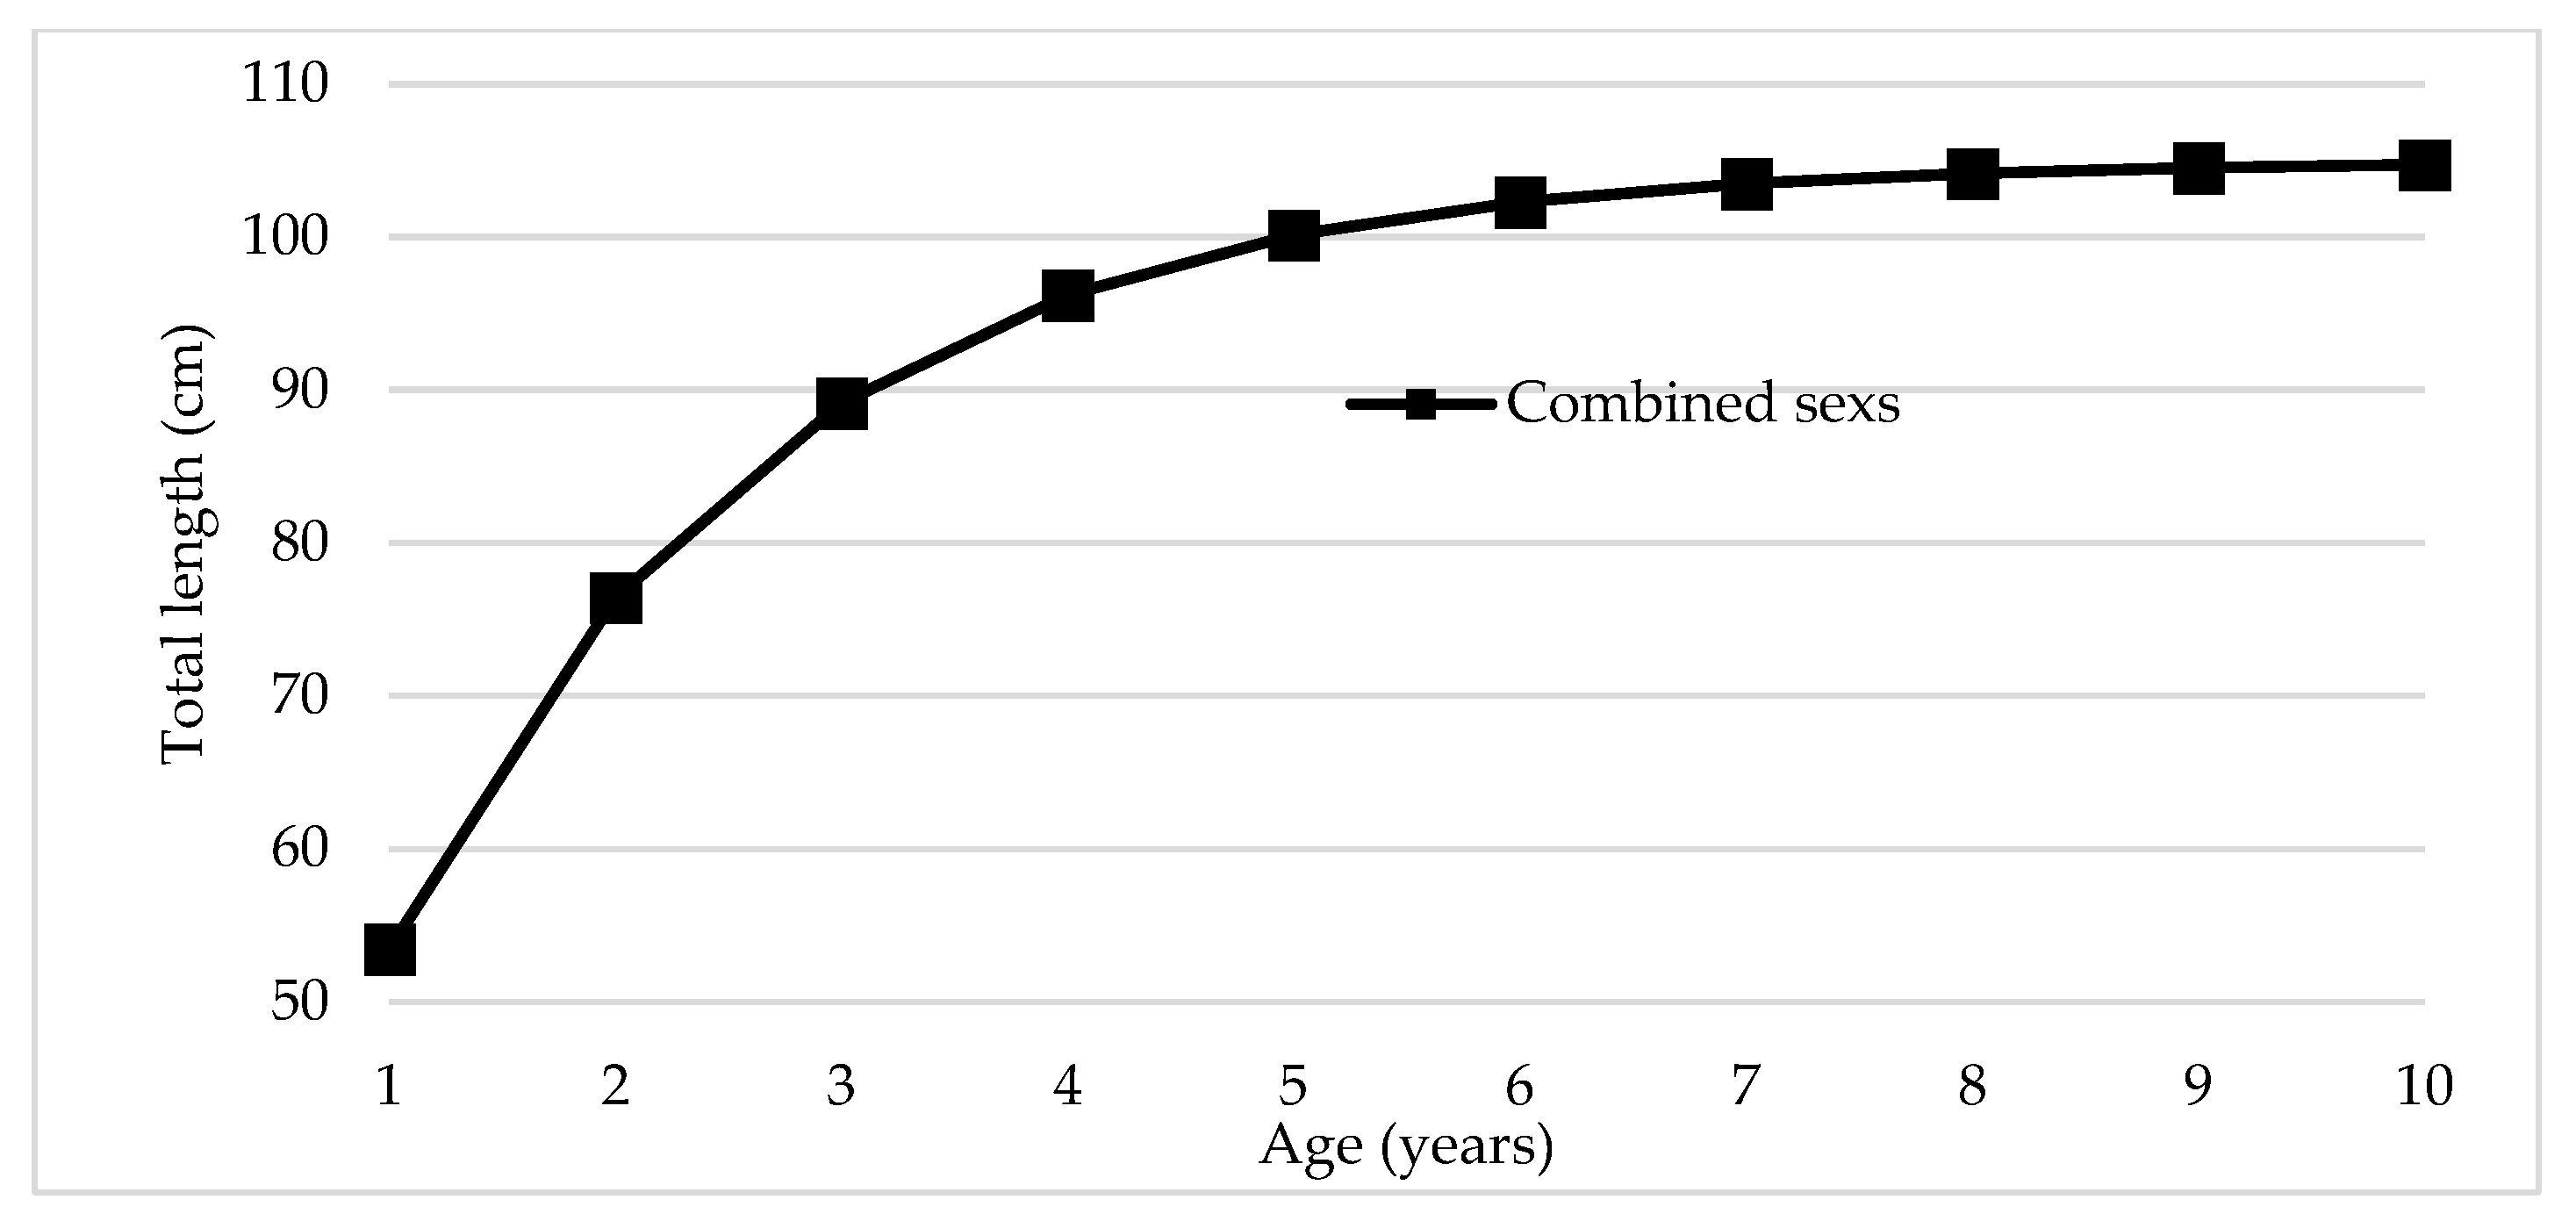
The von Bertalanffy growth curve in length for combined sexes of R. terraenovae showed a pattern of rapid growth during the first years of life, with subsequent gradual deceleration when approaching the asymptotic length (Figure 4). The observed points, corresponding to lengths converted to age (n = 541), were adequately distributed around the fitted curve, indicating a good fit of the model to the data.
During the first 3–4 years, individuals reached approximately 60–70% of their asymptotic length (L∞ = 105 cm), evidencing accelerated growth characteristic of species with a “fast” life history strategy. At 5 years, the mean length was approximately 85 cm, and at 8 years it exceeded 95 cm, with a marked reduction in annual growth rate observed after 6–7 years. The asymptote of 105 cm represents the theoretical maximum length that individuals can reach in the region, although the low representation of organisms >90 cm in the catches (Figure 2) suggests that few individuals fully express their growth potential due to fishing pressure.
Growth parameter estimates are presented in Table 2. ANOVA detected no significant differences between sexes for L∞ (F = 0.144, p = 0.714) nor for k (F = 0.319, p = 0.585); therefore, combined sex parameters were used for mortality analyses. The growth performance index (Ø′ = 3.81) falls within the range reported for the species (3.34–3.86; Table 2).

3.4. Mortality

Mortality estimates for combined sexes are presented in Table 3. The Z values obtained by Jones-van Zalinge (Z3 = Z4 = 4.13 years−1) were higher than those from catch curve and presented lower uncertainty (CIL = 1.05). Mean natural mortality was M = 0.467 years−1 (M1 = 0.461, M2 = 0.473). Mean fishing mortality with lower uncertainty was F = 3.22 years−1 (95% CI: 2.69–3.74).

3.5. Exploitation Rate

The 32 E estimates ranged from 0.42 to 1.21. Two-way ANOVA revealed significant effects of the Z method (F = 6.56, p = 0.002) and F method (F = 4.52, p = 0.001) (Table 4).
The estimates with lowest uncertainty corresponded to combinations with Z3–Z4 and F5–F8 (Table 5), with E values ranging from 0.76 to 0.80 and CIL between 0.05–0.07. One-way ANOVA detected no significant differences among these four estimates (F = 2.57, p = 0.089), yielding a mean value: E = 0.78 (95% CI: 0.745–0.805).
This value significantly exceeds the reference point of E = 0.5 [53], indicating that the population of R. terraenovae in Marine Priority Regions 45 and 46 and in the influence area of the Playa Tortuguera Rancho Nuevo Wetland of International Importance is in a state of severe overexploitation.

4. Discussion

The main finding of this study is the documentation of a state of severe overexploitation (E = 0.78) of R. terraenovae in Priority Marine Regions 45 and 46, a high priority area for conservation under the regime of the Conservation Sector of the Marine Ecological Management Program of the Gulf of Mexico [23]. This result acquires fundamental relevance for fisheries management in the region, since it shows an unsustainable fishing pressure on a key species of the coastal ecosystem. These findings are then discussed in the context of previous studies . the ecological role of R. terraenovae as a medium-high trophic level predator and the consequences of its elimination on the ecosystem structure are analyzed, the implications for the conservation of sea turtles in the Playa Rancho Nuevo Sanctuary are evaluated, recognizing its secondary nature within the general ecological context, and management measures with an ecosystem approach that balance fisheries sustainability with ecological integrity are proposed. Finally, methodological lessons are drawn for the evaluation of artisanal fisheries in contexts of limited data and the limitations of the study are discussed.

4.1. Von Bertalanffy Growth Model

Although the literature has reported that some growth models in sharks and rays, different from the Von Bertalanffy (VBM) model, have provided better adjustments [55,56] the VBM has continued to be adjusted without evaluation of other models [57,58]. But it has also been shown that in small sharks (LT < 100 cm) the model with the best assertion to the growth data has been the VBM [55].

4.2. Interpretation of Size Structure in Relation to Sexual Maturity

The size structure observed in the captures of R. terraenovae shows a trend in the range of 64–68 cm, with an almost total absence of individuals smaller than 50 cm and a scarce representation of specimens larger than 85 cm (Figure 2). To interpret the biological significance of this distribution, it is necessary to contrast it with the values reported in the literature on the birth size and the size of first sexual maturity of the species. In the Gulf of Mexico, the birth size of R. terraenovae has been estimated to be between 30 and 35 cm [16], while the first sexual maturity size for females ranges from 65 to 70 cm [59]. Therefore, the mode of our captures (64–68 cm) is right at the threshold of sexual maturity, suggesting that most of the captured individuals are young adults who have reached or are very close to reaching their first reproduction. The almost total absence of neonates (<50 cm) in the catches indicates that nursery habitats (possibly coastal lagoons or shallow waters) are not being exploited by artisanal longline and gillnet fisheries, or that these individuals are not present in the study area. This spatial segregation by size, also documented in other regions of the Gulf of Mexico [22], has important implications for management: the protection of breeding habitats and the establishment of a minimum catch size above the first maturity size (70 cm TL) are key measures to ensure that individuals have at least one reproductive opportunity before being recruited to the fishery [60].

4.3. Overexploitation of R. terraenovae in Priority Marine Regions 45 and 46

The fishing exploitation rate is an indicator of the exploitation status of a fishery resource that has not lost its validity [61,62,63,64,65,66]. The estimated exploitation rate (E = 0.78) (95% CI: 0.745–0.805) estimated in this study significantly exceeds the reference point of E = 0.5 [54], indicating that the population of R. terraenovae in Marine Priority Regions 45 and 46 and in the area of influence of the Playa Tortuguera Rancho Nuevo Wetland of International Importance is in a state of severe overexploitation.
Likewise, E = 0.78 is comparable to the value of 0.77 reported by Aguirre-García et al. [17] for Campeche, but substantially higher than the values of 0.37–0.39 reported by Worm et al. [18] and Zea-de-la-Cruz [67] for the southern Gulf of Mexico and Veracruz, respectively (Table 6). The estimated fishing mortality (F = 3.22 years−1) is the highest documented for the species in the Gulf of Mexico, reflecting intense fishing pressure in the region. These regional differences could be explained by variations in fishing intensity, selectivity of fishing gear, and local oceanographic features that affect stock productivity [31,68].
Particularly notable is the difference with the study by Bada-Sánchez et al. [30], who reported an exploitation rate of only 0.14 for the Banco de Campeche, suggesting an underexploited population. This discrepancy could be due to methodological differences: Bada-Sánchez et al. [30] used Hoenig’s [69] model modified by Then et al. [70] to estimate M, while we used Pauly’s (1980) [71] method. Additionally, the natural mortality estimated in this study (M = 0.46 years−1) is slightly lower than that reported by Bada-Sánchez et al. [30] (M = 0.50 years−1), but similar to the values documented by other authors for the species in the Gulf of Mexico ([16]: M = 0.39 years−1; [17]: M = 0.39 years−1; [67]: M = 0.27–0.70 years−1). The main difference lies in fishing mortality (F), which in our study (F = 3.22 years−1) is considerably higher than that reported by Bada-Sánchez et al. [30] (F = 0.19 years−1), reflecting substantially higher fishing pressure in Marine Priority Regions 45–46 of Tamaulipas compared to the Bank of Campeche.
It is possible that there are real differences in the status of stocks between regions, which would support the hypothesis of multiple fish stocks in the Gulf of Mexico. Recent studies on size distribution along the Gulf Coast have shown that R. terraenovae populations have a complex spatial structure, with variations in the proportion of juveniles and adults between states [16,22]. This geographic variability underscores the importance of conducting stock assessments at appropriate regional scales, rather than assuming population homogeneity across the Gulf of Mexico. However, the possible spatial structuring of the population of R. terraenovae in the Gulf of Mexico is a topic of debate in the literature. Genetic studies based on Amplified Fragment Length Polymorphism suggest high genetic connectivity and the existence of a single population in the region [72]. However, ecological evidence indicates a differential habitat use by size: while neonates and small juveniles may use coastal lagoons as nursery areas [22], larger adults are predominantly captured in open marine waters ([16]; this study). This apparent contradiction between genetic connectivity and ecological segregation suggests that, although large-scale gene flow exists, populations may be functionally structured at the regional level, which has important implications for fisheries management.
In the specific case of the Bank of Campeche, there could host a population with lower fishing pressure, our results indicate that the population of R. terraenovae in Priority Marine Regions 45–46 is overexploited (E = 0.78) as a result of the intense artisanal fishing pressure in this region of high priority for conservation, confirming the H1 hypothesis.

4.4. Ecological Role of Sharks in the Coastal Ecosystem

Coastal sharks occupy high trophic positions in marine food webs, where their role as top predators generates cascading effects that regulate populations at lower trophic levels and maintain ecosystem structure and stability [73]. Recent studies have shown that elasmobranchs act as critical energy vectors between ecosystems, connecting neritic, oceanic, and deep-sea habitats, promoting ecological resilience in the face of threats such as habitat degradation and climate change [74]. In the northwestern Gulf of Mexico, research on the trophic ecology of juvenile sharks has revealed that their diet is dominated by teleost fish, with ontogenetic and spatial variations associated with changes in prey availability and estuarine environmental conditions [75]. The overexploitation documented in this study (E = 0.78) not only compromises the sustainability of the fishery, but also implies a potential alteration of these ecological interactions in Marine Priority Regions 45 and 46, with consequences not yet assessed on the structure of the coastal ecosystem and the services it provides [76].

4.5. Implications for Sea Turtle Conservation

The sea turtles that nest in the Playa Rancho Nuevo Sanctuary, in particular the olive ridley turtle (Lepidochelys kempii), face a series of anthropogenic threats that are mainly responsible for the decline of their populations, including the loss and degradation of nesting beaches, pollution, bycatch, and the effects of climate change on incubation temperature and food availability [26,27]. Natural predation by sharks, although it occurs occasionally during the hatching season (August–November), does not constitute a significant threat to the population viability of L. kempii. In the case of R. terraenovae, diet studies in the southern Gulf of Mexico indicate that turtle neonates do not represent a relevant component in its diet, which is dominated by small fish and crustaceans [77]. Therefore, although the overexploitation of dogfish shark documented in this study (E = 0.78) may have important ecological implications on the coastal ecosystem, its direct impact on sea turtles is likely minimal. In line with the ecosystem approach to fisheries management, turtle conservation should be addressed through specific measures targeting anthropogenic threats, while the recovery of shark populations is self-justifying, by virtue of their functional role in the structure and stability of the marine community [73,74].

4.6. Biological Consistency of Estimates

Despite the high fishing mortality rates, our growth and natural mortality parameters show biological consistency with what has been reported for the species in other regions. The growth performance index (Ø′ = 3.81) is within the range of 3.34–3.86 documented for R. terraenovae in the Gulf of Mexico [31,50,78]. The M/k = 0.79 ratio (using M = 0.467 years−1 and k = 0.59 years−1 from ELEFAN) approximates the range of 0.5–1.0 typically observed in exploited elasmobranch populations [79,80], and is consistent with the values reported for the species in other locations in the Gulf of Mexico ([16]: M/k = 0.65; [17]: M/k = 0.46–0.57). The estimated asymptotic length (L∞ = 105 cm) is similar to that reported by Zea-de-la-Cruz [67] for Veracruz (104.3 cm) and by Branstetter [81] for Galveston Bay (108 cm). This consistency suggests that, although our fishing mortality values (F = 3.22 years−1) are the highest documented for the species, the natural growth and mortality parameters are biologically plausible and reflect exceptionally intense fishing pressure in Marine Priority Regions 45–46 of Tamaulipas.

4.7. Implications for Management with an Ecosystem Approach in the Conservation Sector

Our results have direct implications for the management of Marine Priority Regions 45 and 46 and the Playa Tortuguera Rancho Nuevo Wetland of International Importance, in line with the objectives of the Conservation Sector of the Marine Ecological Management Program [23] and with the strategies established in the Sanctuary Management Program [26]. Specifically, the latter establishes as a priority action: “Promote before the competent authority the best practices of commercial, coastal and artisanal fishing, for those fisheries that have some negative impact on sea turtle populations” [26]. The R. terraenovae fishery, due to its trophic interaction with neonates, qualifies as a fishery with a potential impact on turtles, although the direction and magnitude of that impact requires further investigation.
Artisanal shark fishing in Priority Marine Regions 45 and 46 is a fundamental economic activity for the coastal communities of La Barra del Tordo, Tepehuajes and Carbonera, where it generates employment and direct and indirect income for numerous families [39]. According to the Rancho Nuevo Beach Sanctuary Management Program [26], coastal and artisanal fishing is the main source of livelihood in these localities, and its continuity depends on the health of fishing resources and the stability of the coastal ecosystem. In this context, any management measures aimed at reducing overexploitation of R. terraenovae must balance conservation objectives with the economic viability of fishing communities, recognizing that the long-term sustainability of the fishery is also a requirement for the social and economic stability of the region [82]. For this reason, the proposed measures—such as minimum sizes, temporary closures and zoning—have been designed considering their feasibility of implementation and their potential to maintain, in the medium term, catch levels within biologically sustainable limits, while protecting fishermen’s livelihoods.
The ecosystem approach to fisheries management (EBFM) explicitly recognizes the need to consider the interactions between target and non-target species, as well as the trophic effects of fisheries [83,84,85]. Within the framework of the Conservation Sector, which seeks to make the protection of ecosystems compatible with the sustainable use of resources, we propose the following integrated management measures for the area:
(a)
Establishment of a legal minimum size (70 cm TL) based on the size of the first sexual maturity of the species [16,59]. This measure allows individuals to reproduce at least once before being recruited into the fishery, contributing to the sustainability of the breeding stock [60].
(b)
Temporary closure during the reproductive period of R. terraenovae (spring–summer), which coincides with the calving period in the Gulf of Mexico [16,86]. This measure aims to reduce fishing mortality of gravid females and neonates at a critical time in the life cycle of the species. While no specific breeding grounds have been identified in the study region, recent research in the southeastern Gulf of Mexico documents the use of coastal lagoons by neonates [16], underscoring the need for telemetry studies to identify priority conservation areas in Tamaulipas.
(c)
Fisheries zoning that establishes temporary or permanent exclusion areas for fishing gear with high bycatch of elasmobranchs, such as gillnets, in areas identified as breeding habitats [21,76]. Although specific breeding areas have not yet been identified in the region, recent research in the southeastern Gulf of Mexico documents the use of coastal lagoons by neonates [16], underscoring the need for telemetry studies to locate these priority areas in Tamaulipas.
(d)
Participatory monitoring with local fishermen to obtain catch time series and evaluate the effect of management measures, within the framework of the recommendations for Marine Priority Region 46, where it is suggested to evaluate the pressure on crab, shrimp and fish species [36]. Experience in other regions shows that participatory monitoring strengthens local governance and improves the acceptance of management measures [87,88].
(e)
Interdisciplinary research to evaluate the real impact of predation by R. terraenovae on turtle neonates, through analysis of stomach contents, telemetry studies and food web models. However, the main justification for the conservation of sharks lies in their functional role as medium-high trophic level predators in the coastal ecosystem [73,74], rather than in their occasional interaction with charismatic species.
(f)
Implementation of best fishing practices as established by the Sanctuary Management Program, including training of fishermen in bycatch turtle release techniques and the adoption of selective fishing gear, as well as the release of juvenile shark individuals caught below the minimum legal size [89].
(g)
Strengthening of surveillance in Rancho Nuevo for the protection of turtles, addressing the identified problem of “lack of surveillance in Rancho Nuevo for the protection of turtles (olive ridley)” [36]. This measure, although targeting turtles, indirectly contributes to the sustainability of the fishery by reducing illegal fishing.
(h)
Support for alternative livelihoods as a strategy to reduce fishing pressure on vulnerable species, recognizing that artisanal fisheries are the livelihood of local communities [90]. Income diversification programs have shown positive results in shark conservation in other regions [90].
(i)
These measures should be implemented through a participatory process involving fishers, fisheries authorities (National Fisheries and Aquaculture Commission) and environmental authorities (National Commission of Natural Protected Areas, CONANP), within the framework of the management councils of natural protected areas and environmental policy instruments such as the Marine Ecological Management Program. Collaborative governance is essential for the success of management strategies in artisanal fisheries [91].

4.8. Lessons for the Assessment of Data-Limited Fisheries in Priority Areas for Conservation

This study is a case of successful application of methods based on size frequencies for the evaluation of an artisanal fishery with limited data in a context of high relevance for conservation (Priority Marine Regions and Wetland of International Importance). Size-based methods are appropriate for artisanal fisheries in priority areas for conservation. Since these methods do not require sacrificing sophisticated organisms or equipment, they are particularly suitable for protected natural areas and priority regions where the impact of research is to be minimized. This is in line with the guidelines established by the CONANP [26], which emphasize that research activities in the Sanctuary must be carried out with the minimum possible disturbance to protected species and their habitats. Several lessons can be drawn from this experience:
Methodological uncertainty can and should be quantified explicitly. By generating multiple estimates using different methods and k-values, and by applying bootstrap to estimate confidence intervals, we were able to identify the most robust combinations (lower LIC) and obtain a point estimate with its corresponding uncertainty. This approach is recommended for all assessments in data-limited fisheries [92,93].
Consistency with comparative indices (Ø′) and theoretical relations (M/k) provides indirect validation. Despite the absence of age-independent validation, the consistency of our growth parameters with those reported in the literature and with the Beverton-Holt invariants [94] suggests that the estimates are biologically plausible.
Participatory monitoring with fishermen is feasible and generates quality data. Collaboration with local fishermen allowed a sample of 541 organisms to be obtained over 16 months, demonstrating that it is possible to generate valuable information even without large investments in monitoring infrastructure.
Size-based methods are appropriate for artisanal fisheries in priority areas for conservation. Since these methods do not require the sacrifice of organisms or sophisticated equipment, they are particularly suitable for protected natural areas and priority regions where the impact of research is sought to be minimized.
The integration of fisheries management and conservation objectives is possible even with limited information. Our study shows that, even in contexts of limited data, it is possible to generate relevant information for decision-making that integrates both fisheries sustainability and the conservation of priority species and the fulfillment of the objectives of the Conservation Sector (confirming H3).

4.9. Limitations of the Study and Future Prospects

We recognize the inherent limitations of the size-frequency-based methods used in this study. These methods assume that the population is steady-state, recruitment is constant, and the sample is representative of the population [40]. Our data come exclusively from landings of artisanal fisheries in La Barra del Tordo, which implies that the size structure observed is influenced by the selectivity of the fishing gear used (longline and gillnets) and by the spatial behavior of the species. Certain components of the population, such as larger sharks or neonates, may occupy different habitats or have movement patterns that make them less vulnerable to artisanal fisheries in the study area, which could bias our estimates of population structure.
In particular, the almost total absence of individuals > 90 cm in catches (Figure 2), despite the fact that previous studies in Tamaulipas have documented the presence of large breeding sharks in the region [16], could be explained by at least two non-exclusive hypotheses: (1) a localized depletion of these individuals due to the high fishing pressure documented in this study (E = 0.78), which would support our main conclusion; or (2) an ontogenetic change in the spatial distribution of the species, where larger individuals could inhabit areas not covered by our samples, such as deeper waters or areas far from artisanal fisheries [31,95]. The absence of telemetry or tagging studies in the region prevents discerning between these two possibilities, underscoring the need for future research to better understand the movement patterns and habitat use of R. terraenovae in the area.
Although we seek to minimize bias through systematic sampling over 16 months, we cannot rule out partial violations of these assumptions.
The absence of age-independent validation (by reading vertebrae) is another limitation, since growth estimates could be influenced by the grouping of data into height classes [96]. In addition, the estimation of M using Pauly’s [53] empirical formula introduces uncertainty, since this equation was developed for teleost fish and its application to elasmobranchs must be interpreted with caution.
Future research should be aimed at: (1) validating age and growth by reading vertebrae and microchemistry analysis to determine population connectivity; (2) to quantify the predation of R. terraenovae on turtle neonates by analysis of stable isotopes and stomach contents; (3) assess the movement and residence of the species in the Priority Marine Regions using acoustic telemetry; (4) to model trophic interactions in the coastal ecosystem using Ecopath or Ecosim models; (5) applying ecological risk assessment models (SCAs) that integrate uncertainty into biological and fisheries parameters; (6) evaluate the status of other elasmobranch species captured in the region, such as Sphyrna tiburo and Carcharhinus acronotus, to determine if they face similar pressures, and (7) in order to address uncertainties about the representativeness of the sample and the spatial structure of the population, it is recommended to implement a tagging–telemetry study (acoustic or satellite) to determine: (1) the home range of R. terraenovae in Priority Marine Regions 45–46; (2) movement patterns between artisanal fishing areas, coastal lagoons (such as those described by Wakida-Kusunoki et al. [22]), and potential nursery areas; and (3) connectivity between different segments of the population in the northern Gulf of Mexico. This type of study would be essential to validate or refute the hypothesis of local adult depletion and to design more effective management measures, such as fishing zoning.

5. Conclusions

This study provides the first quantitative assessment of the population status of R. terraenovae in Marine Priority Regions 45 “La Pesca-Rancho Nuevo” and 46 “Laguna de San Andrés”, and in the influence area of the Playa Tortuguera Rancho Nuevo Wetland of International Importance (Ramsar Site No. 1326), Tamaulipas, demonstrating that it is possible to obtain robust estimates in data-limited fishery contexts in high-priority conservation areas.
The estimated exploitation rate (E = 0.78; 95% CI: 0.745–0.805) significantly exceeds the reference point of E = 0.5, indicating that the population is in a state of severe overexploitation (confirming H1).
The high fishing mortality rates (F = 3.22 years−1) reflect the intense artisanal fishing pressure in these priority regions, where fishermen from communities such as La Barra del Tordo, Tepehuajes, and Carbonera operate, within the framework of the Conservation Sector of the Marine Ecological Zoning Program.
Overexploitation of R. terraenovae has potential implications for the structure and functioning of the coastal ecosystem, given the species’ role as a medium-high trophic level predator. While this includes interactions with other species such as sea turtles, the main rationale for shark conservation lies in their role in maintaining ecological integrity and in supporting the objectives of the Conservation Sector.
This study demonstrates that, despite the limitations inherent to data-limited fisheries, it is possible to generate quantitative information relevant for decision-making through length–frequency-based methods, uncertainty analysis, and validation through comparative indices (confirming H3).
Urgent implementation of ecosystem-based fisheries management in Marine Priority Regions 45 and 46 is required, considering the interactions between the R. terraenovae fishery and sea turtle conservation, including minimum legal sizes (70 cm TL), temporary closures coordinated with the hatching season, fishing zoning, participatory monitoring, and strengthening of surveillance, addressing the specific recommendations of environmental policy instruments.
This study contributes to fulfillment of the objectives of the Conservation Sector of the Gulf of Mexico and Caribbean Sea Marine and Regional Ecological Zoning Program [23] and of the commitments derived from the Ramsar designation of the Playa Tortuguera Rancho Nuevo site, by providing scientific bases to reconcile fisheries exploitation with biodiversity conservation in these priority areas.

Author Contributions

Conceptualization, J.H.R.-C. and S.E.O.-d.l.F.; methodology, J.H.R.-C. and S.E.O.-d.l.F.; software, J.H.R.-C., S.E.O.-d.l.F., J.A.R.-O., U.d.J.B.-M. and J.T.-O.; validation, J.H.R.-C., J.A.R.-O., U.d.J.B.-M., J.A.R.-L. and L.A.V.-O.; formal analysis, J.H.R.-C., S.E.O.-d.l.F. and J.A.R.-L.; investigation, J.H.R.-C., S.E.O.-d.l.F., U.d.J.B.-M. and J.A.R.-L.; resources, J.H.R.-C., S.E.O.-d.l.F., J.A.R.-O., J.T.-O., J.A.R.-L. and L.A.V.-O.; data curation, J.H.R.-C., U.d.J.B.-M., J.T.-O. and L.A.V.-O.; writing—original draft preparation, J.H.R.-C. and S.E.O.-d.l.F.; writing—review and editing, S.E.O.-d.l.F., J.A.R.-O., U.d.J.B.-M. and J.A.R.-L.; visualization, J.H.R.-C., J.A.R.-O., U.d.J.B.-M., J.A.R.-L. and L.A.V.-O.; supervision, J.H.R.-C., J.A.R.-O., U.d.J.B.-M., J.T.-O. and L.A.V.-O.; project administration, J.H.R.-C., J.T.-O. and L.A.V.-O.; funding acquisition, J.H.R.-C., S.E.O.-d.l.F. and L.A.V.-O. All authors have read and agreed to the published version of the manuscript.

Funding

This research received no external funding.

Institutional Review Board Statement

Not applicable. Organisms were obtained directly from artisanal fishery landings in La Barra del Tordo, with the collaboration of local fishermen.

Informed Consent Statement

Not applicable.

Data Availability Statement

The authors will make the raw data that support the conclusions of this article available to others without undue reservation.

Conflicts of Interest

The authors declare no conflicts of interest.

References

  1. FAO. The State of World Fisheries and Aquaculture 2020; Food and Agriculture Organization of the United Nations: Rome, Italy, 2020. [Google Scholar]
  2. Avadí, A.; Acosta-Alba, I. Eco-Efficiency of the Fisheries Value Chains in the Gambia and Mali. Foods 2021, 10, 1620. [Google Scholar] [CrossRef] [Scilit]
  3. Haque, A.B.; Cavanagh, R.D.; Seddon, N. Evaluating artisanal fishing of globally threatened sharks and rays in the Bay of Bengal, Bangladesh. PLoS ONE 2021, 16, e0256146. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  4. Mejía, C.V.; Rodríguez, G.; Tanner, M.K.; Ramírez-González, J.; Moity, N.; Andrade, S.; Paladines, M.J.B.; Cáceres, R.; Castrejón, M.; Pittman, J. Fishing during the “new normality”: Social and economic changes in Galapagos small-scale fisheries due to the COVID-19 pandemic. Marit. Stud. 2022, 21, 193–208. [Google Scholar] [CrossRef] [Scilit]
  5. Hilborn, R.; Ovando, D. Reflections on the success of traditional fisheries management. ICES J. Mar. Sci. 2014, 71, 1040–1046. [Google Scholar] [CrossRef] [Scilit]
  6. Santos, R.; Peixoto, U.I.; Medeiros-Leal, W.; Novoa-Pabon, A.; Pinho, M. Growth Parameters and Mortality Rates Estimated for Seven Data-Deficient Fishes from the Azores Based on Length-Frequency Data. Life 2022, 12, 778. [Google Scholar] [CrossRef] [Scilit]
  7. Tavares, R.; Carreon-Zapiain, M.T.; Perez-Jimenez, J.C. Vulnerability of elasmobranchs caught by artisanal fishery in the Southeastern Caribbean. Reg. Stud. Mar. Sci. 2024, 79, 103851. [Google Scholar] [CrossRef] [Scilit]
  8. Peñaherrera-Palma, C.R.; Chinacalle-Martínez, N.S.; Zamora, W.G.; Jaramillo-Vallejo, S.P.; López-Macías, J.P.; Safady-Mendoza, O.; Bravo-Ormaza, M.E. Reconstructing the spatial and temporal dynamics of Ecuador’s artisanal small-scale fisheries from fishers’ perspective. PLoS ONE 2025, 20, e0338495. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  9. Prince, J.D.; Rufiati, I.; Septiani, W.D.; Kembaren, D.D.; Gough, C.L.A. A novel size-based method for assessing the spawning potential ratio of data-poor octopus fisheries. Front. Mar. Sci. 2025, 12, 1647742. [Google Scholar] [CrossRef] [Scilit]
  10. Klaoudatos, D.; Theocharis, A. Methodologies for Data-Poor Fisheries Assessment in the Mediterranean Basin: Status, Challenges, and Future Directions. Fishes 2025, 11, 22. [Google Scholar] [CrossRef] [Scilit]
  11. Canales, C.M.; Punt, A.E.; Mardones, M. Can a length-based pseudo-cohort analysis (LBPA) using multiple catch length-frequencies provide insight into population status in data-poor situations? Fish. Res. 2021, 234, 105810. [Google Scholar] [CrossRef] [Scilit]
  12. Prince, J.D.; Wilcox, C.; Hall, N. How to estimate life history ratios to simplify data-poor fisheries assessment. ICES J. Mar. Sci. 2023, 80, 2619–2629. [Google Scholar] [CrossRef] [Scilit]
  13. Sandin, S.A.; French, B.J.; Zgliczynski, B.J. Emerging insights on effects of sharks and other top predators on coral reefs. Emerg. Top. Life Sci. 2022, 6, 57–65. [Google Scholar] [CrossRef] [Scilit]
  14. Lubitz, N.; Abrantes, K.; Crook, K.; Currey-Randall, L.M.; Chin, A.; Sheaves, M.; Fitzpatrick, R.; Martins, A.B.; Bierwagen, S.; Miller, I.B.; et al. Trophic ecology shapes spatial ecology of two sympatric predators, the great hammerhead shark (Sphyrna mokarran) and bull shark (Carcharhinus leucas). Front. Mar. Sci. 2023, 10, 1274275. [Google Scholar] [CrossRef] [Scilit]
  15. Cortés, E. Life history patterns and correlations in sharks. Rev. Fish. Sci. 2000, 8, 299–344. [Google Scholar] [CrossRef] [Scilit]
  16. Márquez-Farias, J.F.; Castillo-Geniz, J.L. Fishery biology and demography of the Atlantic sharpnose shark, Rhizoprionodon terraenovae, in the southern Gulf of Mexico. Fish. Res. 1998, 39, 183–198. [Google Scholar] [CrossRef] [Scilit]
  17. Aguirre-García, B.; Medina-Quej, A.; López-García, A. Análisis de la pesquería artesanal del “cazón de ley” Rhizoprionodon terraenovae (Richardson, 1836) en Campeche, México. In Proceedings of the 60th Gulf and Caribbean Fisheries Institute, Punta Cana, Dominican Republic, 5–9 November 2007; Gulf and Caribbean Fisheries Institute: Miami, FL, USA, 2004; Volume 60, pp. 153–160. [Google Scholar]
  18. Worm, B.; Davis, B.; Kettemer, L.; Ward-Paige, C.A.; Chapman, D.; Heithaus, M.R.; Kessel, S.T.; Gruber, S.H. Global catches, exploitation rates, and rebuilding options for sharks. Mar. Policy 2013, 40, 194–204. [Google Scholar] [CrossRef] [Scilit]
  19. Walker, T.I. Management measures. In Management Techniques for Elasmobranch Fisheries; Musick, J.A., Bonfil, R., Eds.; FAO Fisheries Technical Paper No. 474; Food and Agriculture Organization of the United Nations: Rome, Italy, 2005; pp. 216–242. [Google Scholar]
  20. Dulvy, N.K.; Fowler, S.L.; Musick, J.A.; Cavanagh, R.D.; Kyne, P.M.; Harrison, L.R.; Carlson, J.K.; Davidson, L.N.; Fordham, S.V.; Francis, M.P.; et al. Extinction risk and conservation of the world’s sharks and rays. eLife 2014, 3, e00590. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  21. Driggers, W.B.; Campbell, D.M.; Jones, C.M.; Hannon, K.M.; Hoffmayer, E.R.; Sulikowski, J.A. Spatial variability in the fecundity of Atlantic sharpnose sharks (Rhizoprionodon terraenovae) in the northern Gulf of Mexico. Fish. Bull. 2020, 118, 51–62. [Google Scholar] [CrossRef] [Scilit]
  22. Wakida-Kusunoki, A.T.; Anislado-Tolentino, V.; Del Moral-Flores, L.F. Unusual presence of atlantic sharpnose shark (Rhizoprionodon terraenovae) neonates in a coastal lagoon in southeast Gulf of Mexico. Novit. Caribaea 2025, 62–69. [Google Scholar] [CrossRef] [Scilit]
  23. DOF. Acuerdo Por el Que se Expide la Parte Marina del Programa de Ordenamiento Ecológico Marino y Regional del Golfo de México y Mar Caribe; Diario Oficial de la Federación: Mexico City, Mexico, 2012. [Google Scholar]
  24. CONANP. Ficha Informativa de los Humedales de Ramsar—Santuario Playa Rancho Nuevo; Comisión Nacional de Áreas Naturales Protegidas: Ciudad de México, México, 2004. [Google Scholar]
  25. IUCN. The IUCN Red List of Threatened Species, Version 2023-1; International Union for Conservation of Nature: Gland, Switzerland, 2023. [Google Scholar]
  26. CONANP. Programa de Manejo del Santuario Playa Rancho Nuevo; Comisión Nacional de Áreas Naturales Protegidas: Ciudad de México, México, 2014. [Google Scholar]
  27. Pilcher, N.J.; Antonopoulou, M.; Rodriguez-Zarate, C.J. Marine turtle nest predation. Endanger. Species Res. 2021, 45, 123–136. [Google Scholar]
  28. Bashir, Z.; Abdullah, M.M.; Ghaffar, M.A.; Rusli, M.U. Exclusive predation of sea turtle hatchlings by juvenile blacktip reef sharks Carcharhinus melanopterus at a turtle nesting site in Malaysia. J. Fish Biol. 2020, 97, 1876–1879. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  29. Oñate-Casado, J.; Booth, D.T.; Vandercamere, K.; Sakhalkar, S.P.; Rusli, M.U. Offshore Dispersal and Predation of Sea Turtle Hatchlings I: A Study of Hawksbill Turtles at Chagar Hutang Turtle Sanctuary, Malaysia. Ichthyol. Herpetol. 2021, 109, 180–187. [Google Scholar] [CrossRef] [Scilit]
  30. Bada-Sánchez, E.; Pérez-Jiménez, J.C.; Méndez-Loaeza, I. Estado del stock pesquero del cazón tutzún Rhizoprionodon terraenovae (Richardson, 1836) en el Banco de Campeche. In Proceedings of the VII Simposio Nacional de Tiburones y Rayas, Puerto Vallarta, Jalisco, México, 18–22 April 2016; Anislado-Tolentino, V., Pérez-Jiménez, J.C., Cabrera-Sánchez, M.G., Eds.; Sociedad Mexicana de Peces Cartilaginosos, A.C.: México D.F., México, 2016; pp. 53–55. [Google Scholar]
  31. Loefer, J.K.; Sedberry, G.R. Life history of the Atlantic sharpnose shark (Rhizoprionodon terraenovae) (Richardson, 1836) off the southeastern United States. Fish. Bull. 2003, 101, 75–88. [Google Scholar]
  32. Nikolic, N.; Devloo-Delva, F.; Bailleul, D.; Noskova, E.; Rougeux, C.; Delord, C.; Borsa, P.; Liautard-Haag, C.; Hassan, M.; Marie, A.D.; et al. Stepping up to genome scan allows stock differentiation in the worldwide distributed blue shark Prionace glauca. Mol. Ecol. 2022, 32, 1000–1019. [Google Scholar] [CrossRef] [Scilit]
  33. Leone, A.; Arnaud-Haond, S.; Babbucci, M.; Bargelloni, L.; Coscia, I.; Damalas, D.; Delord, C.; Franch, R.; Garibaldi, F.; Macias, D.; et al. Population Genomics of the Blue Shark, Prionace glauca, Reveals Different Populations in the Mediterranean Sea and the Northeast Atlantic. Evol. Appl. 2024, 17, e70005. [Google Scholar] [CrossRef] [Scilit]
  34. Chhina, A.K.; Abhari, N.; Mooers, A.; Lewthwaite, J.M. Linking the spatial and genomic structure of adaptive potential for conservation management: A review. Genome 2024, 67, 403–423. [Google Scholar] [CrossRef] [Scilit]
  35. Massa, P.; Leitão, H.G.; Manousaki, T.; Cariani, A.; Svardal, H.; Tsaparis, D.; Cannas, R.; Zane, L.; De Pooter, T.; Spedicato, M.T.; et al. Genomic insights into the population structure and adaptive variation of Mullus barbatus in the Mediterranean Sea. BMC Evol. Biol. 2025, 25, 101. [Google Scholar] [CrossRef] [Scilit]
  36. Arriaga, L.; Vázquez, E.; González, J.; Jiménez, R.; Muñoz, E.; Aguilar, V. Regiones Marinas Prioritarias de México; Comisión Nacional para el Conocimiento y Uso de la Biodiversidad (CONABIO): México D.F., México, 1998. [Google Scholar]
  37. Caballero-Rico, F.C.; Roque-Hernández, R.V.; Cano, R.d.l.G.; Arvizu-Sánchez, E. Challenges for the Integrated Management of Priority Areas for Conservation in Tamaulipas, México. Sustainability 2022, 14, 494. [Google Scholar] [CrossRef] [Scilit]
  38. INAPESCA. Boletín Hidrometeorológico—Temperatura Superficial del Mar; Instituto Nacional de Pesca: Ciudad de México, México, 2013. [Google Scholar]
  39. SEMARNAT. Diagnóstico del Sector Pesquero en la Costa Sur de Tamaulipas; Secretaría de Medio Ambiente y Recursos Naturales, Delegación Tamaulipas: Ciudad Victoria, Mexico, 2014. [Google Scholar]
  40. Sparre, P.; Venema, S.C. Introducción a la Evaluación de Recursos Pesqueros Tropicales. Parte 1. Manual; FAO Documento Técnico de Pesca No. 306.1, Rev. 2; Food and Agriculture Organization of the United Nations: Rome, Italy, 1998. [Google Scholar]
  41. Hordyk, A.; Ono, K.; Valencia, S.; Loneragan, N.; Prince, J. A novel length-based empirical estimation method of spawning potential ratio (SPR), and tests of its performance, for small-scale, data-poor fisheries. World Conference on Stock Assessment Methods for Sustainable Fisheries. ICES J. Mar. Sci. 2015, 72, 217–231. [Google Scholar] [CrossRef] [Scilit]
  42. Zar, J.H. Biostatistical Analysis, 5th ed.; Prentice Hall: Upper Saddle River, NJ, USA, 2010. [Google Scholar]
  43. Ricker, W.E. Computation and Interpretation of Biological Statistics of Fish Populations. Bull. Fish. Res. Board Can. 1977, 41, 154–155. [Google Scholar] [CrossRef] [Scilit]
  44. Walpole, R.E.; Myers, R.H.; Myers, S.L.; Ye, K. Probability & Statistics for Engineers & Scientists, 9th ed.; Pearson: Boston, MA, USA, 2012. [Google Scholar]
  45. Chen, Y.; Jackson, D.A.; Harvey, H.H. A Comparison of von Bertalanffy and Polynomial Functions in Modelling Fish Growth Data. Can. J. Fish. Aquat. Sci. 1992, 49, 1228–1235. [Google Scholar] [CrossRef] [Scilit]
  46. von Bertalanffy, L. A quantitative theory of organic growth. Hum. Biol. 1938, 10, 181–213. [Google Scholar]
  47. Gayanilo, F.C.; Sparre, P.; Pauly, D. FAO-ICLARM Stock Assessment Tools II (FiSAT II). Revised Version, User’s Guide; FAO Computerized Information Series (Fisheries) No. 8; Food and Agriculture Organization of the United Nations: Rome, Italy, 2005. [Google Scholar]
  48. Pauly, D. Fish population dynamics in tropical waters: A manual for use with programmable calculators. In ICLARM Studies and Reviews; ICLARM: Manila, Philippines, 1984; Volume 8, pp. 1–325. [Google Scholar]
  49. Efron, B.; Tibshirani, R.J. An Introduction to the Bootstrap; Chapman & Hall: New York, NY, USA, 1993. [Google Scholar]
  50. Pauly, D.; Munro, J.L. Once more on the comparison of growth in fish and invertebrates. Fishbyte 1984, 2, 21. [Google Scholar]
  51. Pauly, D. Growth performance in fishes: Rigorous description of patterns as a basis for understanding causal mechanisms. Aquabyte 1991, 4, 3–6. [Google Scholar]
  52. Jones, R.; van Zalinge, N.P. Estimations of mortality rate and population size for shrimp in Kuwait waters. Kuwait Bull. Mar. Sci. 1981, 2, 273–288. [Google Scholar]
  53. Pauly, D. On the interrelationships between natural mortality, growth parameters, and mean environmental temperature in 175 fish stocks. ICES J. Mar. Sci. 1980, 39, 175–192. [Google Scholar] [CrossRef] [Scilit]
  54. Gulland, J.A. Manual de Métodos para la Evaluación de las Poblaciones de Peces; Acribia: Zaragoza, Spain, 1971. [Google Scholar]
  55. Liu, K.M.; Wu, C.B.; Joung, S.J.; Tsai, W.P.; Su, K.Y. Multi-model approach on growth estimation and association with life history trait for elasmobranchs. Front. Mar. Sci. 2021, 8, 591692. [Google Scholar] [CrossRef] [Scilit]
  56. Caña-Hernández, S.; Lara-Mendoza, R.E.; Mendoza-Carranza, M.; Pérez-Jiménez, J.C. Using a multimodel approach to determine the age and growth of an endangered small shark species in the southern Gulf of Mexico. Reg. Stud. Mar. Sci. 2023, 60, 102836. [Google Scholar] [CrossRef] [Scilit]
  57. Dureuil, M.; Aeberhard, W.H.; Dowd, M.; Pardo, S.A.; Whoriskey, F.G.; Worm, B. Reliable growth estimation from mark–recapture tagging data in elasmobranchs. Fish. Res. 2022, 256, 106488. [Google Scholar] [CrossRef] [Scilit]
  58. Talwar, B.S.; Bradley, D.; Berry, C.; Bond, M.E.; Bouyoucos, I.A.; Brooks, A.M.L.; Fields, C.Y.A.; Gallagher, A.J.; Guttridge, T.L.; Guttridge, A.E.; et al. Estimated life-history traits and movements of the Caribbean reef shark (Carcharhinus perezi) in The Bahamas based on tag-recapture data. Mar. Biol. 2022, 169, 55. [Google Scholar] [CrossRef] [Scilit]
  59. Oviedo-Pérez, J.L.; Zea-de-la-Cruz, H.; Aguirre-Villaseño, D.H.; Meiners-Mandujano, C.; Jiménez-Badillo, L.; González-Ocaranza, L. Talla de madurez sexual del tiburón Rhizoprionodon terraenovae en Veracruz, México. Cienc. Pesq. 2014, 22, 37–45. [Google Scholar]
  60. Musick, J.A. Criteria to Define Extinction Risk in Marine Fishes: The American Fisheries Society Initiative. Fisheries 1999, 24, 6–14. [Google Scholar] [CrossRef] [Scilit]
  61. Hashemi, S.A.; Doustdar, M.; Ghasemzadeh, J.; Gholampour, A. Length-based fishery status of skipjack tuna, Katsuwonus pelamis (Linnaeus, 1758) (Teleostei: Scombridae: Scombrinae) in the northern waters of the Oman Sea (Iran). Iran. J. Ichthyol. 2021, 8, 160–169. [Google Scholar]
  62. Mehanna, S.F.; Samy-Kamal, M. Population Dynamics Parameters and Exploitation Status of 55 Commercial Species in Egyptian Red Sea Fisheries: A Key to Sustainable Fisheries. Fishes 2024, 9, 255. [Google Scholar] [CrossRef] [Scilit]
  63. Rahman, O.; Laboni, T.A.; Khatun, M.S.; Rahman, A.; Islam, A.; Rahman, M.; Parvin, M.F.; Abedin, J.; Hossain, Y. Estimating the growth parameters, exploitation rate, biomass and maximum sustainable yield of long whisker catfish Mystus gulio (Hamilton, 1822) in the coastal waters from southwestern Bangladesh. Heliyon 2024, 10, e29788. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  64. Aladawi, U.; Majeed, S.; Al-Anboori, I.; Amin, S.M.N. Assessment of Exploited Stock and Management Implications of Kingfish (Scomberomorus commerson) in the Omani Waters. Fishes 2025, 10, 589. [Google Scholar] [CrossRef] [Scilit]
  65. Das, D.; Priester, R.; Soares, J.; Macena, B.; Fontes, J.; Afonso, P. Nearshore essential habitat of threatened sharks around a temperate oceanic island. Mar. Ecol. Prog. Ser. 2025, 766, 73–90. [Google Scholar] [CrossRef] [Scilit]
  66. Hashemi, S.A.; Doustdar, M.; Al Kindi, A.; Dutta, S. Assessment of Population Dynamics and Fishery Exploitation of Narrow-Barred Spanish Mackerel (Scomberomorus commerson) in Iranian Waters. Oceans 2025, 6, 55. [Google Scholar] [CrossRef] [Scilit]
  67. la Cruz, H.Z.-D.; Tovar-Ávila, J.; Meiners-Mandujano, C.; Jiménez-Badillo, L.; Oviedo-Pérez, J.L. Determining potential management strategies for the elasmobranchs bycatch of the Mexican shrimp trawl fishery of the Gulf of Mexico through a vulnerability analysis. Reg. Stud. Mar. Sci. 2021, 42, 101626. [Google Scholar] [CrossRef] [Scilit]
  68. Mukherji, S.; Simpfendorfer, C.; Dowling, N.; Krueck, N.C. Assessing mechanisms of intrinsic vulnerability in sharks occupying different marine environments. Biodivers. Conserv. 2026, 35, 31. [Google Scholar] [CrossRef] [Scilit]
  69. Hoenig, J.M. Empirical use of longevity data to estimate mortality rates. Fish. Bull. 1983, 82, 898–903. [Google Scholar]
  70. Then, A.Y.; Hoenig, J.M.; Hall, N.G.; Hewitt, D.A. Evaluating the predictive performance of empirical estimators of natural mortality rate using information on over 200 fish species. ICES J. Mar. Sci. 2014, 72, 82–92. [Google Scholar] [CrossRef] [Scilit]
  71. Pauly, D. Some simple methods for the assessment of tropical fish stocks. In FAO Fisheries Technical Paper; FAO: Rome, Italy, 1980; Volume 234, p. 52. [Google Scholar]
  72. Suárez-Moo, P.d.J.; Rocha-Olivares, A.; Zapata-Pérez, O.; Quiroz-Moreno, A.; Sánchez-Teyer, L.F. High genetic connectivity in the Atlantic sharpnose shark, Rhizoprionodon terraenovae, from the southeast Gulf of Mexico inferred from AFLP fingerprinting. Fish. Res. 2013, 147, 338–343. [Google Scholar] [CrossRef] [Scilit]
  73. Su, H.; Zhou, L.; Xie, P. What can we learn from the loss of sharks? Trends Ecol. Evol. 2025, 40, 531–533. [Google Scholar] [CrossRef] [Scilit]
  74. Shipley, O.N.; Matich, P.; Hussey, N.E.; Brooks, A.M.L.; Chapman, D.; Frisk, M.G.; Guttridge, A.E.; Guttridge, T.L.; Howey, L.A.; Kattan, S.; et al. Energetic connectivity of diverse elasmobranch populations—Implications for ecological resilience. Proc. R. Soc. B Biol. Sci. 2023, 290, 20230262. [Google Scholar] [CrossRef] [Scilit]
  75. TinHan, T.C.; Wells, R.J.D. Spatial and Ontogenetic Patterns in the Trophic Ecology of Juvenile Bull Sharks (Carcharhinus leucas) From the Northwest Gulf of Mexico. Front. Mar. Sci. 2021, 8, 664316. [Google Scholar] [CrossRef] [Scilit]
  76. Matich, P.; Bigelow, C.L.; Chambers, B.; Dodds, J.J.; Hebert, J.A.; Lemieux, A.; Pittman, C.M.; Trapp, J.; Bianco, B.; Cadena, C.P.; et al. Delineation of blacktip shark (Carcharhinus limbatus) nursery habitats in the north-western Gulf of Mexico. J. Fish Biol. 2022, 101, 236–248. [Google Scholar] [CrossRef] [Scilit]
  77. Viana-Morayta, J.E.; Torres-Rojas, Y.E.; Camalich-Carpizo, J. Diet shifts of Rhizoprionodon terraenovae from the southern Gulf of Mexico: Possible scenario by temperature changes. Lat. Am. J. Aquat. Res. 2020, 48, 406–420. [Google Scholar] [CrossRef] [Scilit]
  78. SEDAR. SEDAR 13—Small Coastal Shark Complex, Atlantic Sharpnose, Blacknose, Bonnethead, and Finetooth Shark Stock Assessment Report; Southeast Data, Assessment, and Review: North Charleston, SC, USA, 2007. [Google Scholar]
  79. Prince, J.; Hordyk, A.; Valencia, S.R.; Loneragan, N.; Sainsbury, K. Revisiting the concept of Beverton–Holt life-history invariants with the aim of informing data-poor fisheries assessment. ICES J. Mar. Sci. 2014, 72, 194–203. [Google Scholar] [CrossRef] [Scilit]
  80. Cortés, E. Perspectives on the intrinsic rate of population increase of elasmobranchs and consequences for sustainable management. Mar. Freshw. Res. 2016, 67, 1843–1852. [Google Scholar]
  81. Branstetter, S. Age and Growth Validation of Newborn Sharks Held in Laboratory Aquaria, with Comments on the Life History of the Atlantic Sharpnose Shark, Rhizoprionodon terraenovae. Copeia 1987, 1987, 291–300. [Google Scholar] [CrossRef] [Scilit]
  82. Béné, C.; Arthur, R.; Norbury, H.; Allison, E.H.; Beveridge, M.; Bush, S.; Campling, L.; Leschen, W.; Little, D.; Squires, D.; et al. Contribution of Fisheries and Aquaculture to Food Security and Poverty Reduction: Assessing the Current Evidence. World Dev. 2016, 79, 177–196. [Google Scholar] [CrossRef] [Scilit]
  83. Perryman, H.A.; Hansen, C.; Howell, D.; Olsen, E. A Review of Applications Evaluating Fisheries Management Scenarios through Marine Ecosystem Models. Rev. Fish. Sci. Aquac. 2021, 29, 800–835. [Google Scholar] [CrossRef] [Scilit]
  84. Woods, P.J.; Macdonald, J.I.; Bárðarson, H.; Bonanomi, S.; Boonstra, W.J.; Cornell, G.; Cripps, G.; Danielsen, R.; Färber, L.; Ferreira, A.S.A.; et al. A review of adaptation options in fisheries management to support resilience and transition under socio-ecological change. ICES J. Mar. Sci. 2021, 79, 463–479. [Google Scholar] [CrossRef] [Scilit]
  85. Craig, J.K.; Link, J.S. It is past time to use ecosystem models tactically to support ecosystem-based fisheries management: Case studies using Ecopath with Ecosim in an operational management context. Fish Fish. 2023, 24, 381–406. [Google Scholar] [CrossRef] [Scilit]
  86. Parsons, G.R.; Hoffmayer, E.R. Seasonal changes in the distribution and availability of the Atlantic sharpnose shark Rhizoprionodon terraenovae in the north central Gulf of Mexico. Copeia 2005, 2005, 913–919. [Google Scholar] [CrossRef] [Scilit]
  87. Ayala, B.; Aranda-Fragoso, A.; Castillo, A.; Basurto, X.; Nenadovic, M. Presentación en la conferencia IASC 2025 sobre gobernanza de pesquerías artesanales en el Pacífico Central Mexicano. In Proceedings of the IASC 2025 XX Biennial Conference, Amherst, MA, USA, 16–20 June 2025. [Google Scholar]
  88. PANORAMA. Fortalecimiento de la Gestión Pesquera a Través de Redes Colectivas (México). 2024. Available online: https://panorama.solutions/es/solution/fortalecimiento-de-la-gestion-pesquera-traves-de-redes-colectivas (accessed on 24 February 2026).
  89. O’FArrell, H.B.; Babcock, E.A.; McCarthy, K.J. Bycatch mitigation for commonly caught shark species in the Gulf of Mexico reef bottom longline fishery. Mar. Coast. Fish. 2024, 16, 10310. [Google Scholar] [CrossRef] [Scilit]
  90. Shidqi, R.A.; Sari, D.R.; Alopen, J.; Bang, Y.M.; Arianto, I.; Kopong, P.N.S.; Td, V.G.; Smulders, E.; Booth, H. Designing and evaluating alternative livelihoods for shark conservation: A case study on thresher sharks in Alor Island, Indonesia. Oryx 2025, 59, 19–30. [Google Scholar] [CrossRef] [Scilit]
  91. Aranda-Fragoso, A.; Castillo, A.; Coronado, E. Pesca artesanal en la costa sur de Jalisco: Reflexiones sobre su investigación y manejo. Soc. Ambient. 2023, 1–31. [Google Scholar] [CrossRef] [Scilit]
  92. Hilborn, R.; Walters, C.J. Quantitative Fisheries Stock Assessment: Choice, Dynamics and Uncertainty; Chapman and Hall: New York, NY, USA, 1992. [Google Scholar]
  93. Punt, A.E.; Butterworth, D.S.; de Moor, C.L.; De Oliveira, J.A.A.; Haddon, M. Management strategy evaluation: Best practices. Fish Fish. 2014, 17, 303–334. [Google Scholar] [CrossRef] [Scilit]
  94. Beverton, R.J.H.; Holt, S.J. A review of the lifespans and mortality rates of fish in nature, and their relation to growth and other physiological characteristics. In Ciba Foundation Symposium—The Lifespan of Animals (Colloquia on Ageing); John Wiley & Sons, Ltd.: Chichester, UK, 1959; Volume 5, pp. 142–180. [Google Scholar]
  95. Carlson, J.K.; Baremore, I.E. Changes in biological parameters of Atlantic sharpnose shark Rhizoprionodon terraenovae in the Gulf of Mexico: Evidence for density-dependent growth and maturity? Mar. Freshw. Res. 2003, 54, 227–234. [Google Scholar] [CrossRef] [Scilit]
  96. Campana, S.E. Accuracy, precision and quality control in age determination, including a review of the use and abuse of age validation methods. J. Fish Biol. 2001, 59, 197–242. [Google Scholar] [CrossRef]
Figure 1. Location of the study area in Marine Priority Regions 45 “La Pesca-Rancho Nuevo” and 46 “Laguna de San Andrés”, Tamaulipas, Mexico. The red box indicates the sampling area in La Barra del Tordo, municipality of Aldama, within the area of influence of the Playa Tortuguera Rancho Nuevo Wetland of International Importance (Ramsar Site No. 1326). The dotted lines delimit the Priority Marine Regions according to the Marine Ecological Management Program of the Gulf of Mexico and the Caribbean Sea [23].
Fishes 11 00268 g001
Figure 2. Frequency distribution of total lengths of R. terraenovae caught by artisanal fisheries in Marine Priority Regions 45–46 and the influence area of the Playa Tortuguera Rancho Nuevo Wetland of International Importance, Tamaulipas, Mexico (November 2018—February 2020): (a) females (n = 260), (b) males (n = 281), and (c) combined sexes (n = 541). Bars represent the relative frequency (%) per 2 cm length interval.
Fishes 11 00268 g002
Figure 3. Power model fitting of the total length-eviscerated weight relationship for R. terraenovae in Marine Priority Regions 45–46, Tamaulipas, Mexico (n = 541). Panels show data distribution for females (a), males (b), and combined sexes (c). Dashed lines represent the model W = aLb (parameters in Table 1).
Fishes 11 00268 g003
Figure 4. Von Bertalanffy growth curve in length for combined sexes of R. terraenovae in Marine Priority Regions 45–46, Tamaulipas, Mexico. Squares represent observed lengths converted to age (n = 541). The continuous line shows the fitted model (parameters in Table 2).
Fishes 11 00268 g004
Table 1. Estimated parameters of the total length-eviscerated weight relationship for R. terraenovae in Marine Priority Regions 45–46, Tamaulipas, Mexico. Coefficients of the model W = a·Lb are presented with their standard errors (SE), coefficient of determination (r2), and t-test results for the isometry hypothesis (H0: b = 3).
Groupna (×10−3)SE(a)bSE(b)r2t (b vs. 3)dLpGrowth Type
Females2606.20.20132.860.11050.90561.2302580.219Isometric
Males2815.00.19742.920.10830.90540.7162790.474Isometric
Combined sexes5415.60.14042.890.07700.90501.3825390.167Isometric
Table 2. Von Bertalanffy growth model parameters for R. terraenovae in Marine Priority Regions 45 and 46 and the influence area of the Playa Tortuguera Rancho Nuevo Wetland of International Importance.
GroupMethodL∞ (cm)95% CI L∞k (Years−1)95% CI kt0 (yr)95% CI t0Ø′
FemalesELEFAN I97.994.2–101.60.380.28–0.48−0.313−0.440–−0.2423.56
MalesELEFAN I100.894.8–106.80.450.40–0.50−0.261−0.302–−0.2293.66
Combined sexesELEFAN I105.0100.0–110.00.590.53–0.65−0.195−0.221–−0.1743.81
Combined sexesShepherd105.0-0.78-−0.152-3.93
Table 3. Estimates of total (Z), natural (M), and fishing (F) mortality for R. terraenovae (combined sexes) in Marine Priority Regions 45 and 46 and the influence area of the Playa Tortuguera Rancho Nuevo Wetland of International Importance.
ParameterMethod/CombinationValue95% CIr2CIL
Z1Curva captura (kELEFAN)2.721.86–3.590.951.73
Z2Curva captura (kShepherd)3.602.46–4.740.952.28
Z3Jones-van Zalinge (kELEFAN)4.133.60–4.650.981.05
Z4Jones-van Zalinge (kShepherd)4.133.60–4.650.981.05
M1Pauly (kELEFAN)0.46---
M2Pauly (kShepherd)0.47---
F5Z3 - M13.302.77–3.82-1.05
F6Z3 - M23.132.61–3.65-1.05
F7Z4 - M13.302.77–3.82-1.05
F8Z4 - M23.132.61–3.65-1.05
Table 4. Point estimates and confidence intervals of the exploitation rate for the sharpnose shark (R. terraenovae) in Aldama, Tamaulipas, estimated by the quotient between fishing mortality (F) and total mortality (Z) parameter values, obtained by various methods.
FZ1 (r2 = 0.95)Z2 (r2 = 0.95)Z3 y Z4 (r2 = 0.98)
θ ^ CI θ ^ CI θ ^ CI
LLULLLULLLUL
F10.700.550.770.530.420.580.460.290.59
F20.630.460.720.480.350.550.420.240.56
F31.020.881.090.770.660.830.670.450.84
F40.960.791.040.720.600.790.630.410.81
F51.211.491.060.921.130.810.80.770.82
F61.151.41.020.871.060.770.760.720.79
F71.211.491.060.921.130.810.80.770.82
F81.151.41.020.871.060.770.760.720.79
θ ^ = Point estimate; CI = Confidence interval; LL = Lower limit; UL = Upper limit.
Table 5. Selected exploitation rate (E) estimates with lowest uncertainty.
CombinationZFE95% CI ECIL
E(5,3)Z3 (4.13)F5 (3.30)0.800.77–0.820.05
E(6,3)Z3 (4.13)F6 (3.13)0.760.72–0.790.07
E(7,4)Z4 (4.13)F7 (3.30)0.800.77–0.820.05
E(8,4)Z4 (4.13)F8 (3.13)0.760.72–0.790.07
Mean--0.780.745–0.8050.06
Table 6. Comparison of R. terraenovae parameters reported in this study and the literature.
AuthorYearRegionL∞ (cm)k (Years−1)ZMFE
This study2026RMP 45–46, Tamps. (Conservation Sector)105.00.594.130.463.220.78
Bada-Sánchez et al.2016Campeche Bank--0.700.500.190.14
Worm et al.2013Southern Gulf of México-----0.37
Zea de la Cruz2012Veracruz Central104.30.441.090.27–0.700.430.39
Aguirre-García et al.2004Campeche114.90.181.670.391.280.77
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.