1. Introduction
The use of pesticides in tree fruit production has evolved substantially over recent decades in response to increasing societal, environmental, and regulatory pressures. Although alternative pest management strategies based on genetics, physical barriers, or biological control have been developed, orchard protection still relies predominantly on foliar spraying. However, conventional spray applications present major limitations, including spray drift, exposure of operators and bystanders, and reduced efficacy in large or dense canopies where target coverage is difficult to achieve [
1,
2]. The presence of plant protection products (PPPs) in the atmosphere and its consequences have emerged in the field of research and expertise and, more recently since the mid-2010s, in public opinion. This issue covers the problem of air contamination by PPPs and the consequences of exposure of populations. Indeed, people living near crop fields may be exposed to plant protection products emitted in the atmosphere and transported downwind. The risks are related to spray drift of the liquid droplets at the time of treatment or the atmospheric dispersion of the fraction of pesticide being volatilized after application.
The evaluation of PPP concentrations in the atmosphere in their various forms and distances was extensively studied [
3,
4,
5]. Major determinants of resident exposure in the vicinity of PPP applications include the drift reducing performance of the spraying equipment, the effects of artificial or natural structures, the effect of adjuvants, and the meteorological conditions during the application [
6]. Extensive studies were conducted in Europe such as PROPULPP in Belgium [
5], OBO in the Netherlands [
7] and more recently CAPRIV in France [
8] in order to better relate the causality of exposure and the role of risk mitigation measures provided by low drift nozzles or hedgerows.
In this context, there is a growing interest in alternative delivery systems that could improve the precision of the application while reducing environmental contamination. One such approach is trunk injection, also referred to as endotherapy, which consists of introducing plant protection products (PPPs) directly into the tree’s vascular system. This method enables systemic redistribution of active ingredients to target organs while minimizing off-target losses. Research on trunk injection in fruit growing systems has expanded in North America since the 2010s, notably through studies conducted on avocado orchards by the University of California [
9], on apple and pear orchards by Michigan State University [
1,
10] and on citrus by the University of Florida [
11]. In France, research conducted since 2015 through several projects, has explored the potential of trunk microinjection as an alternative orchard protection strategy. Expected benefits include eliminating spray drift, reducing the number of applications, improving accessibility to difficult plots (e.g., sloping orchards or waterlogged soil), and developing protection itineraries adapted to diverse orchard contexts.
Tree injection is not a novel concept. Historical records describe injection practices dating back to the Middle Ages, and Leonardo da Vinci reported experimental trunk injections in fruit trees in the 15th century [
12]. Interests in these injection techniques increased among scientists during the 20th century, notably for the management of Dutch elm disease in the 1970s [
13]. Since the early 2000s, trunk injection techniques have been widely adopted in forestry and ornamental arboriculture, supported by advances in application devices and formulation design, leading to reliable pest control results under high infestation pressure [
12]. Today, numerous trunk-injected products are authorized in many countries for the protection of forest, ornamental and urban trees.
One of the main limitations traditionally associated with trunk injection is the need to drill holes into the trunk, which may cause mechanical injury and raise concerns regarding tree health [
14]. To overcome this constraint, microinjection systems that do not require prior drilling have been developed. These devices allow for penetration of the wood and product introduction in a single step, thereby reducing physical damage. In France, the PREAMISSE project (“PRotEction des Arbres par MicroInjection SécuriSEe” 2015–2019) first evaluated this innovative microinjection approach on several models, including the pine processionary moth, grapevine downy and powdery mildews, apple scab, the rosy apple aphid, and the chestnut codling moth. Among the results and knowledge gained from this first French project, the importance of plant species and wood morphology has been clearly demonstrated. The optimization of the technique must be carried out on a species-by-species basis, taking into account tree physiology (particularly the vascular system anatomy) as well as tree size. Although these factors cannot be modified, they must be considered in order to adapt the method to the specific characteristics of each plant species [
15].
To overcome compartmentalization phenomena and ensure optimal transfer and distribution of injected compounds within the tree, the number of injection points, their positioning on the trunk, and needle size must be carefully adjusted. Trials conducted have allowed for refinement of the technique for apple trees (four injection points for mature trees), kiwifruit (four injection points), and for chestnut and walnut trees (one injection point per 10 cm of trunk circumference). This initial study also highlighted the importance of selecting the appropriate active substance for injection. The results indicated that preference should be given to more hydrophilic substances with a log Kow below 3. The octanol–water partition coefficient (log Kow) reflects the lipophilicity of organic compounds and provides an indication of the ability of active substances to be transported within the transpiration stream.
Similarly, formulation characteristics are of critical importance. In France, only one commercial product specifically formulated for trunk injection is currently authorized (REVIVE II, emamectin benzoate, SYNGENTA), for the use against red palm weevil and horse chestnut leaf miner. Consequently, most trials were conducted using commercial products originally designed for spray applications. This highlighted the challenges associated with solid formulations requiring dissolution in water (with variable solubility and potential crystallization issues), as well as formulations with high viscosity, which limit the movement of the injected solution within the sap [
15].
Furthermore, promising biological efficacy results obtained in orchards have encouraged further investigations by CTIFL (Centre Technique Interprofessionnel Fruits et Légumes) and CETEV (Centre d’Etudes Techniques pour l’EnVironnement) within the MISPA project (“MicroInjection Sécurisée pour la Protection des Arbres” 2022-2024). This project focused on seven models: apple scab
Venturia inaequalis and rosy apple aphids
Dysaphis plantaginea in apple orchards, fruit rots
Gnomoniopsis sp. and fruit borers
Cydia splendana,
Pammene fasciana in chestnut orchards, codling moth
Cydia pomonella and husk fly
Rhagoletis completa in nut orchards, bacterial canker
Pseudomonas syringae pv. in kiwi orchards. The objectives of the MISPA project were (i) to generate reference data on the agronomic performance of plant protection products applied through trunk microinjection in selected tree crop models; (ii) to assess the safety of this application method with respect to both tree health and consumer safety; and (iii) to analyze the benefits and constraints of this technique based on various indicators, including biological efficacy, reduction in field interventions, and ease of implementation. Overall, within the framework of this project, significant efficacy has been achieved against insect pests. With regards to diseases, efficacy varies considerably and does not yet meet commercial acceptability thresholds. For the various species studied—apple, chestnut, kiwi and walnut trees—the wound resilience after trunk microinjection has been demonstrated. After one growing season, most of the ports had closed. After two seasons, the bark and wood had recovered their normal structure and xylem had recovered its capacity to transport sap [
16]. This article focuses on the study conducted on rosy apple aphids.
The rosy apple aphid,
Dysaphis plantaginea Passerini, is one of the most damaging pests in apple orchards. It is widely distributed across temperate apple-growing regions in Europe, North America, and parts of Asia, where it represents a major constraint to sustainable apple production. This species is characterized by early spring colonization, with eggs hatching at temperatures as low as 4.5 °C, and by rapid population growth from April to June [
17]. Infestations cause severe leaf curling, shoot deformation, and fruit distortion, resulting in significant yield and quality losses. Economic damage thresholds are often low, as even small colonies can induce irreversible fruit deformation early in the season. In addition, prolonged aphid activity may reduce carbohydrate reserves, negatively affecting flowering and productivity in the following season. In recent years, control failures have been increasingly reported in French apple-growing regions, driven by favorable climatic conditions for aphid development and a reduced availability of authorized insecticides. These failures are also associated with the development of insecticide resistance and the disruption of biological control due to non-selective plant protection practices.
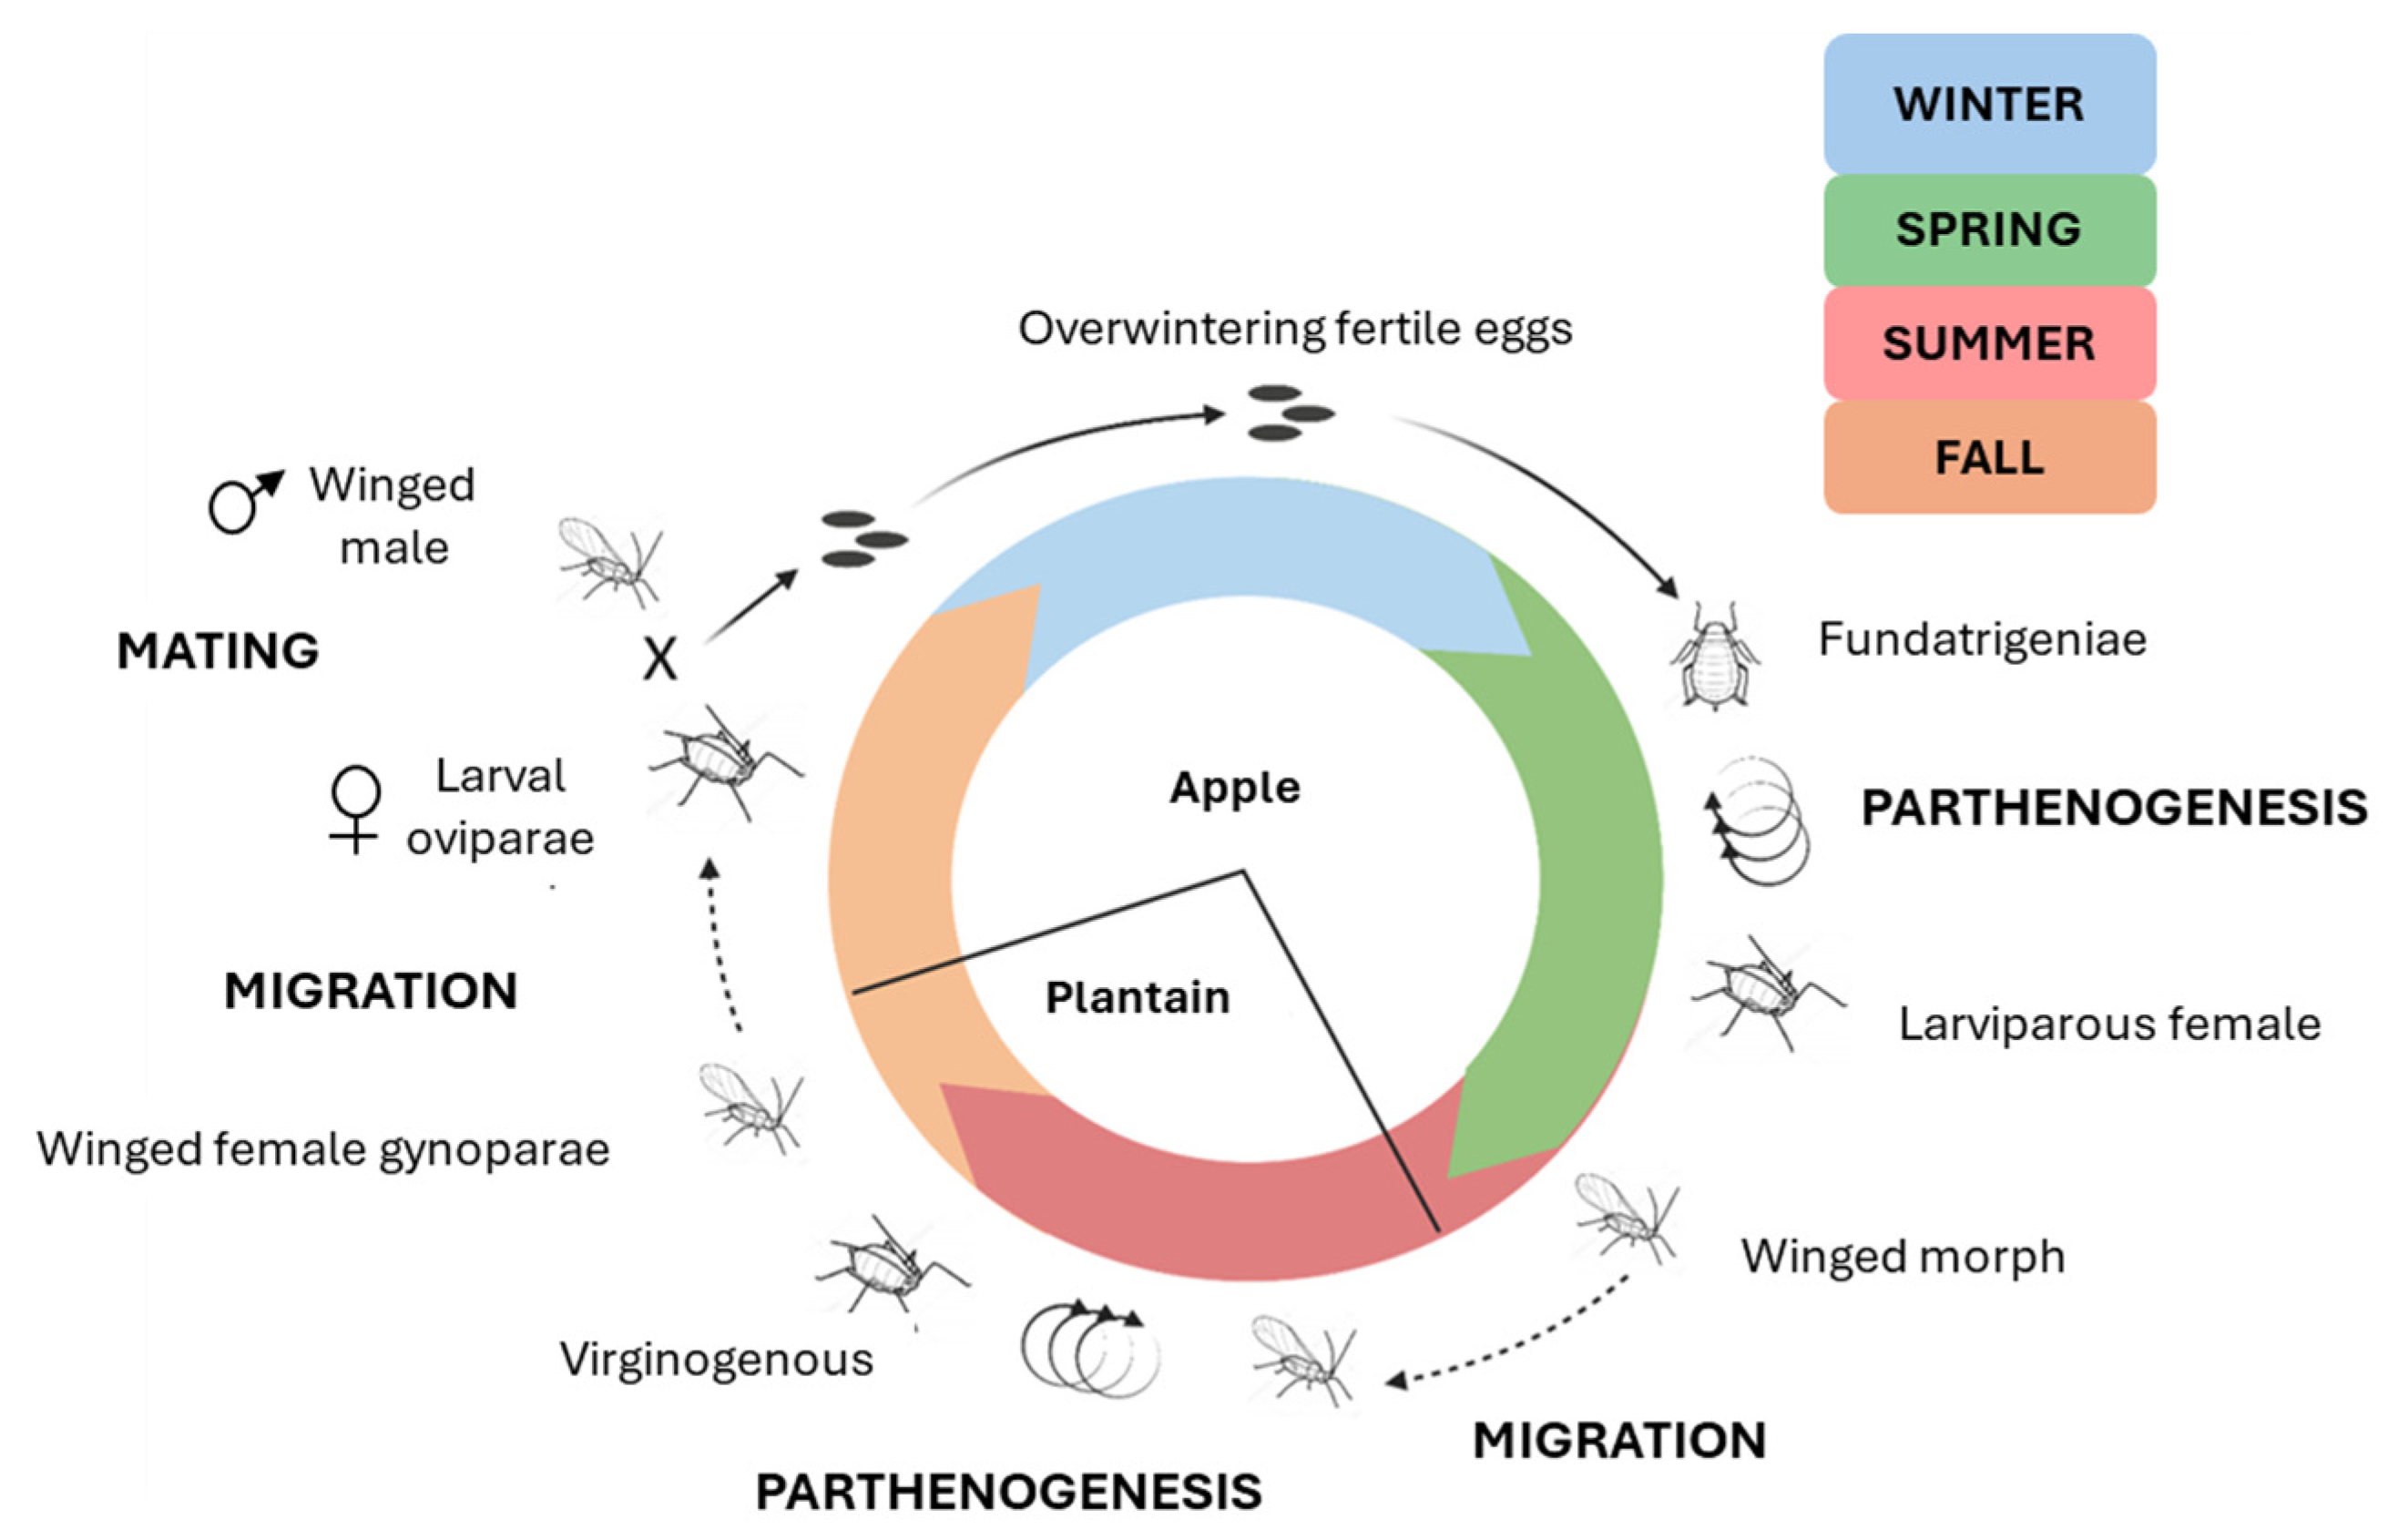
Dysaphis plantaginea has a holocyclic life cycle involving two host plants: apple (
Malus domestica) as the primary host and plantain (
Plantago lanceolata) as the secondary host [
18,
19] (
Figure 1). Overwintering eggs are laid on apple bark near buds and hatch in early spring. The resulting fundatrices give rise to several generations of wingless females before winged migrants appear in early summer and colonize plantain. During this phase, population dynamics are strongly influenced by temperature, host plant phenology, and natural enemies such as parasitoids (e.g.,
Aphidius spp.) and predators (e.g., syrphids and coccinellids). In autumn, gynoparous females and males return to apple trees, where mating occurs and overwintering eggs are laid, completing the cycle.
Effective management of
Dysaphis plantaginea requires disruption of this life cycle at key stages, particularly during egg hatching and early spring colonization, as well as during the autumn return flight to apple trees [
20]. In conventional orchards, control strategies rely on multiple foliar insecticide applications timed to phenological stages, including mineral oils at bud break, flonicamid before flowering, and spirotetramat after petal fall. In organic farming systems, mineral oils and azadirachtin-based products are used, although azadirachtin currently benefits only from temporary derogations for use on pome fruits in France. Autumn strategies in organic orchards may also include clay applications or early defoliation to limit aphid return.
Given these constraints, trunk microinjection represents a promising alternative for managing rosy apple aphid while reducing reliance on foliar sprays. The present study aimed to evaluate the efficacy of trunk microinjection of five PPPs—azadirachtin, flonicamid, spirotetramat, lambda-cyhalothrin, and deltamethrin—for the control of Dysaphis plantaginea in apple orchards. The specific objectives were (i) to assess the effectiveness of microinjected PPPs in reducing aphid infestation levels and associated damage, and (ii) to better understand efficiencies or inefficiencies by quantifying residues in different tissues at key points in the cycle of Dysaphis plantaginea.
2. Materials and Methods
2.1. Plant Material
The study was conducted at the CTIFL experimental site (Centre Technique Interprofessionnel Fruits et Légumes) of Lanxade in Dordogne in southwestern France 44°50′45.1″ N 0°25′17.9″ E. Trees used for this study were apple trees (Malus domestica), variety Ariane grafted on M9 EMLA rootstock planted in winter 2004/2005. The orchard had a density of 2500 trees per hectare with a distance of 4 m between rows and 1 m between plants in the row. The trees were pruned into axes and had an average height of 4 m. The trunks had an average circumference of 27.4 cm ± 3.4 cm measured at 60 cm from the ground. The experiment was conducted as a complete randomized design. The treatments have been monitored since fall 2022 and have evolved over time with annual adjustments. Each treatment involved at least four replications, with each replication comprising four consecutive trees on which observations were made. As the injections were carried out individually on each tree, no “border” trees were required between replicates. However, border rows on either side of the trial acted as a screen between the trial and the rest of the plot (limiting the drift of spray treatments applied to the rest of the plot). No insecticide against Dysaphis plantaginea was applied during the time of evaluation. Irrigation was of the drip type.
2.2. Trees Injections
Five commercial products containing different active substances were tested (
Table 1) with different temporal protection strategies considering
Dysaphis plantaginea cycle: TEPPEKI (flonicamid, ISK Biosciences Europe N.V., Diegem, Belgium), NEEMAZAL (azadirachtine, Andermatt France SAS, Bassussarry, France), MOVENTO (spirotetramat, Bayer, Lyon, France), LAMBDASTAR (lambda-cyhalothrin, Life Scientific Ltd., Dublin, Ireland), DECIS PROTECH (deltamethrin, Bayer, Lyon, France). No commercial product targeting the rosy apple aphid is authorized in France for injection use. The products tested in this study were therefore not formulated for injection (usual use is by spraying). In addition, the device included an untreated control with no injected trees. Application rates were determined based on the indications for use of registered commercial products, including the dose per hectare per application and the maximum number of applications allowed per year. The annual dose per hectare (dose per application × number of applications) was adjusted to the tree density (2500 trees ha
−1). Microinjections were performed using a volume of 1 mL per injection point. For apple trees, four injection points per tree were applied to ensure optimal distribution of active compounds within the canopy. Injected solutions consisted of water dilutions containing a defined proportion of the commercial product. Their administration, following this established protocol, was designed to reproduce the doses authorized for conventional spray applications.
A separate plot, excluded from the experimental design and referred to as the reference plot, was monitored for comparison purposes in order to assess the effectiveness of a conventional spray-based protection program. On this reference plot, the spray program consisted of two applications of SOKALCIARBO (aluminum silicate, Société Kaolinière Armoricaine, Quessoy, France) applied in autumn after harvest, followed by one application of OVIPHYT (paraffin oil, CAS 8042-47-5, Comptoir Commercial des Lubrifiants, Le Meux, France) at the end of winter. Subsequently, between late March and early June, the following treatments were applied in sequence: one application of MAVRIK JET (tau-fluvalinate and pirimicarb, Adama, Suresnes, France), one application of TEPPEKI (flonicamid, ISK Biosciences Europe N.V., Diegem, Belgium), one application of MOVENTO (spirotetramat, Bayer, Lyon, France), and a final application of TEPPEKI (flonicamid, ISK Biosciences Europe N.V., Diegem, Belgium).
Following injection, the compounds enter the xylem sap stream, which consists primarily of water. To reach foliar targets, they must be transported to the leaves via the transpiration stream. A prerequisite for this transport is that the compounds are sufficiently water-soluble and hydrophilic to avoid adsorption onto lipophilic components, such as lignin, encountered along their pathway. Trunk injection also enables compounds to bypass several lipid barriers. As the compounds are directly introduced into the vascular tissues, only their transport within the sap flow needs to be considered. Compounds with low octanol–water partition coefficients (log Kow) are therefore expected to be readily translocated via the xylem sap. In contrast, lipophilic compounds with high log Kow values may undergo adsorption onto xylem vessel walls.
The active substances evaluated in this study exhibited a wide range of log Kow values, suggesting differing theoretical translocation capacities: 0.3 for flonicamid (TEPPEKI), 1.09 for azadirachtin (NEEMAZAL), 2.5 for spirotetramat (MOVENTO), 6.2 for deltamethrin (DECIS PROTECH), and 7 for lambda-cyhalothrin (LAMBDASTAR). These five products are formulated differently. NEEMAZAL and DECIS PROTECH are Emulsifiable Concentrates (EC formulation), TEPPEKI is Dispersible Granule (WG formulation), MOVENTO is Suspension Concentrate (SC) and LAMBDASTAR is Capsule Suspension (CS).
2.3. Tested Strategies
The strategies tested are in line with the pest cycle and have evolved over the years based on annual results. The experimental design was iteratively refined by incorporating annual results and feedback from project partners. In the first year, the objective was to compare an intensified strategy with two injections per aphid cycle (S2: 1 injection in fall + 1 injection in spring) to a reduced strategy with a single spring injection (S3: 1 injection in spring). In the second year, the design was expanded to include an additional reduced strategy (S1) consisting of a single fall injection (S1: 1 injection in fall). The purpose of injecting the product in the fall was to disrupt the return flight of the rosy apple aphid (disrupting nutrition, the reproductive cycle, and therefore egg laying by females). Early application in spring aimed to impact populations emerging from eggs laid in the fall and the offspring of this population. In this study, three strategies were tested (
Table 2).
Microinjections were performed using the Wedgle Direct Inject® device made by ArborSystem, Omaha, NE, USA, equipped with needles improved by CETEV. The needles used measured 2 mm diameter and 3.8 cm length. These needles were inserted directly into the xylem to deliver 1 mL of the prepared solution per injection point. Considering the circumference of the trunks, four points per tree were necessary and positioned evenly around the trunk (North, East, South and West sides) approximately 30 to 60 cm above the ground surface, between the graft union and the lowest branches. A total of 4 mL per tree was microinjected (1 mL multiplied by four injection points).
2.4. Treatments Effects on Dysaphis plantaginea
Observations were made in relation to
Dysaphis plantaginea cycle (
Figure 1). At the end of winter, an initial estimate of the egg population level was made. This involved collecting 20 bud-bearing twigs of 10 cm per replication and observing the presence of eggs using a binocular magnifying glass (ZEISS, Oberkochen, Deutschland). The eggs are oval and very often located at the base of the buds or on bud scales. The number of eggs per twig was counted and the value was expressed as a percentage of twigs with at least one egg counted. In the spring, after flowering in May, observations consisted of counting the number of shoots affected by at least one aphid colony per tree. All the trees were observed from the lowest branches to the highest with the use of a motorized platform.
2.5. Active Ingredients Detection
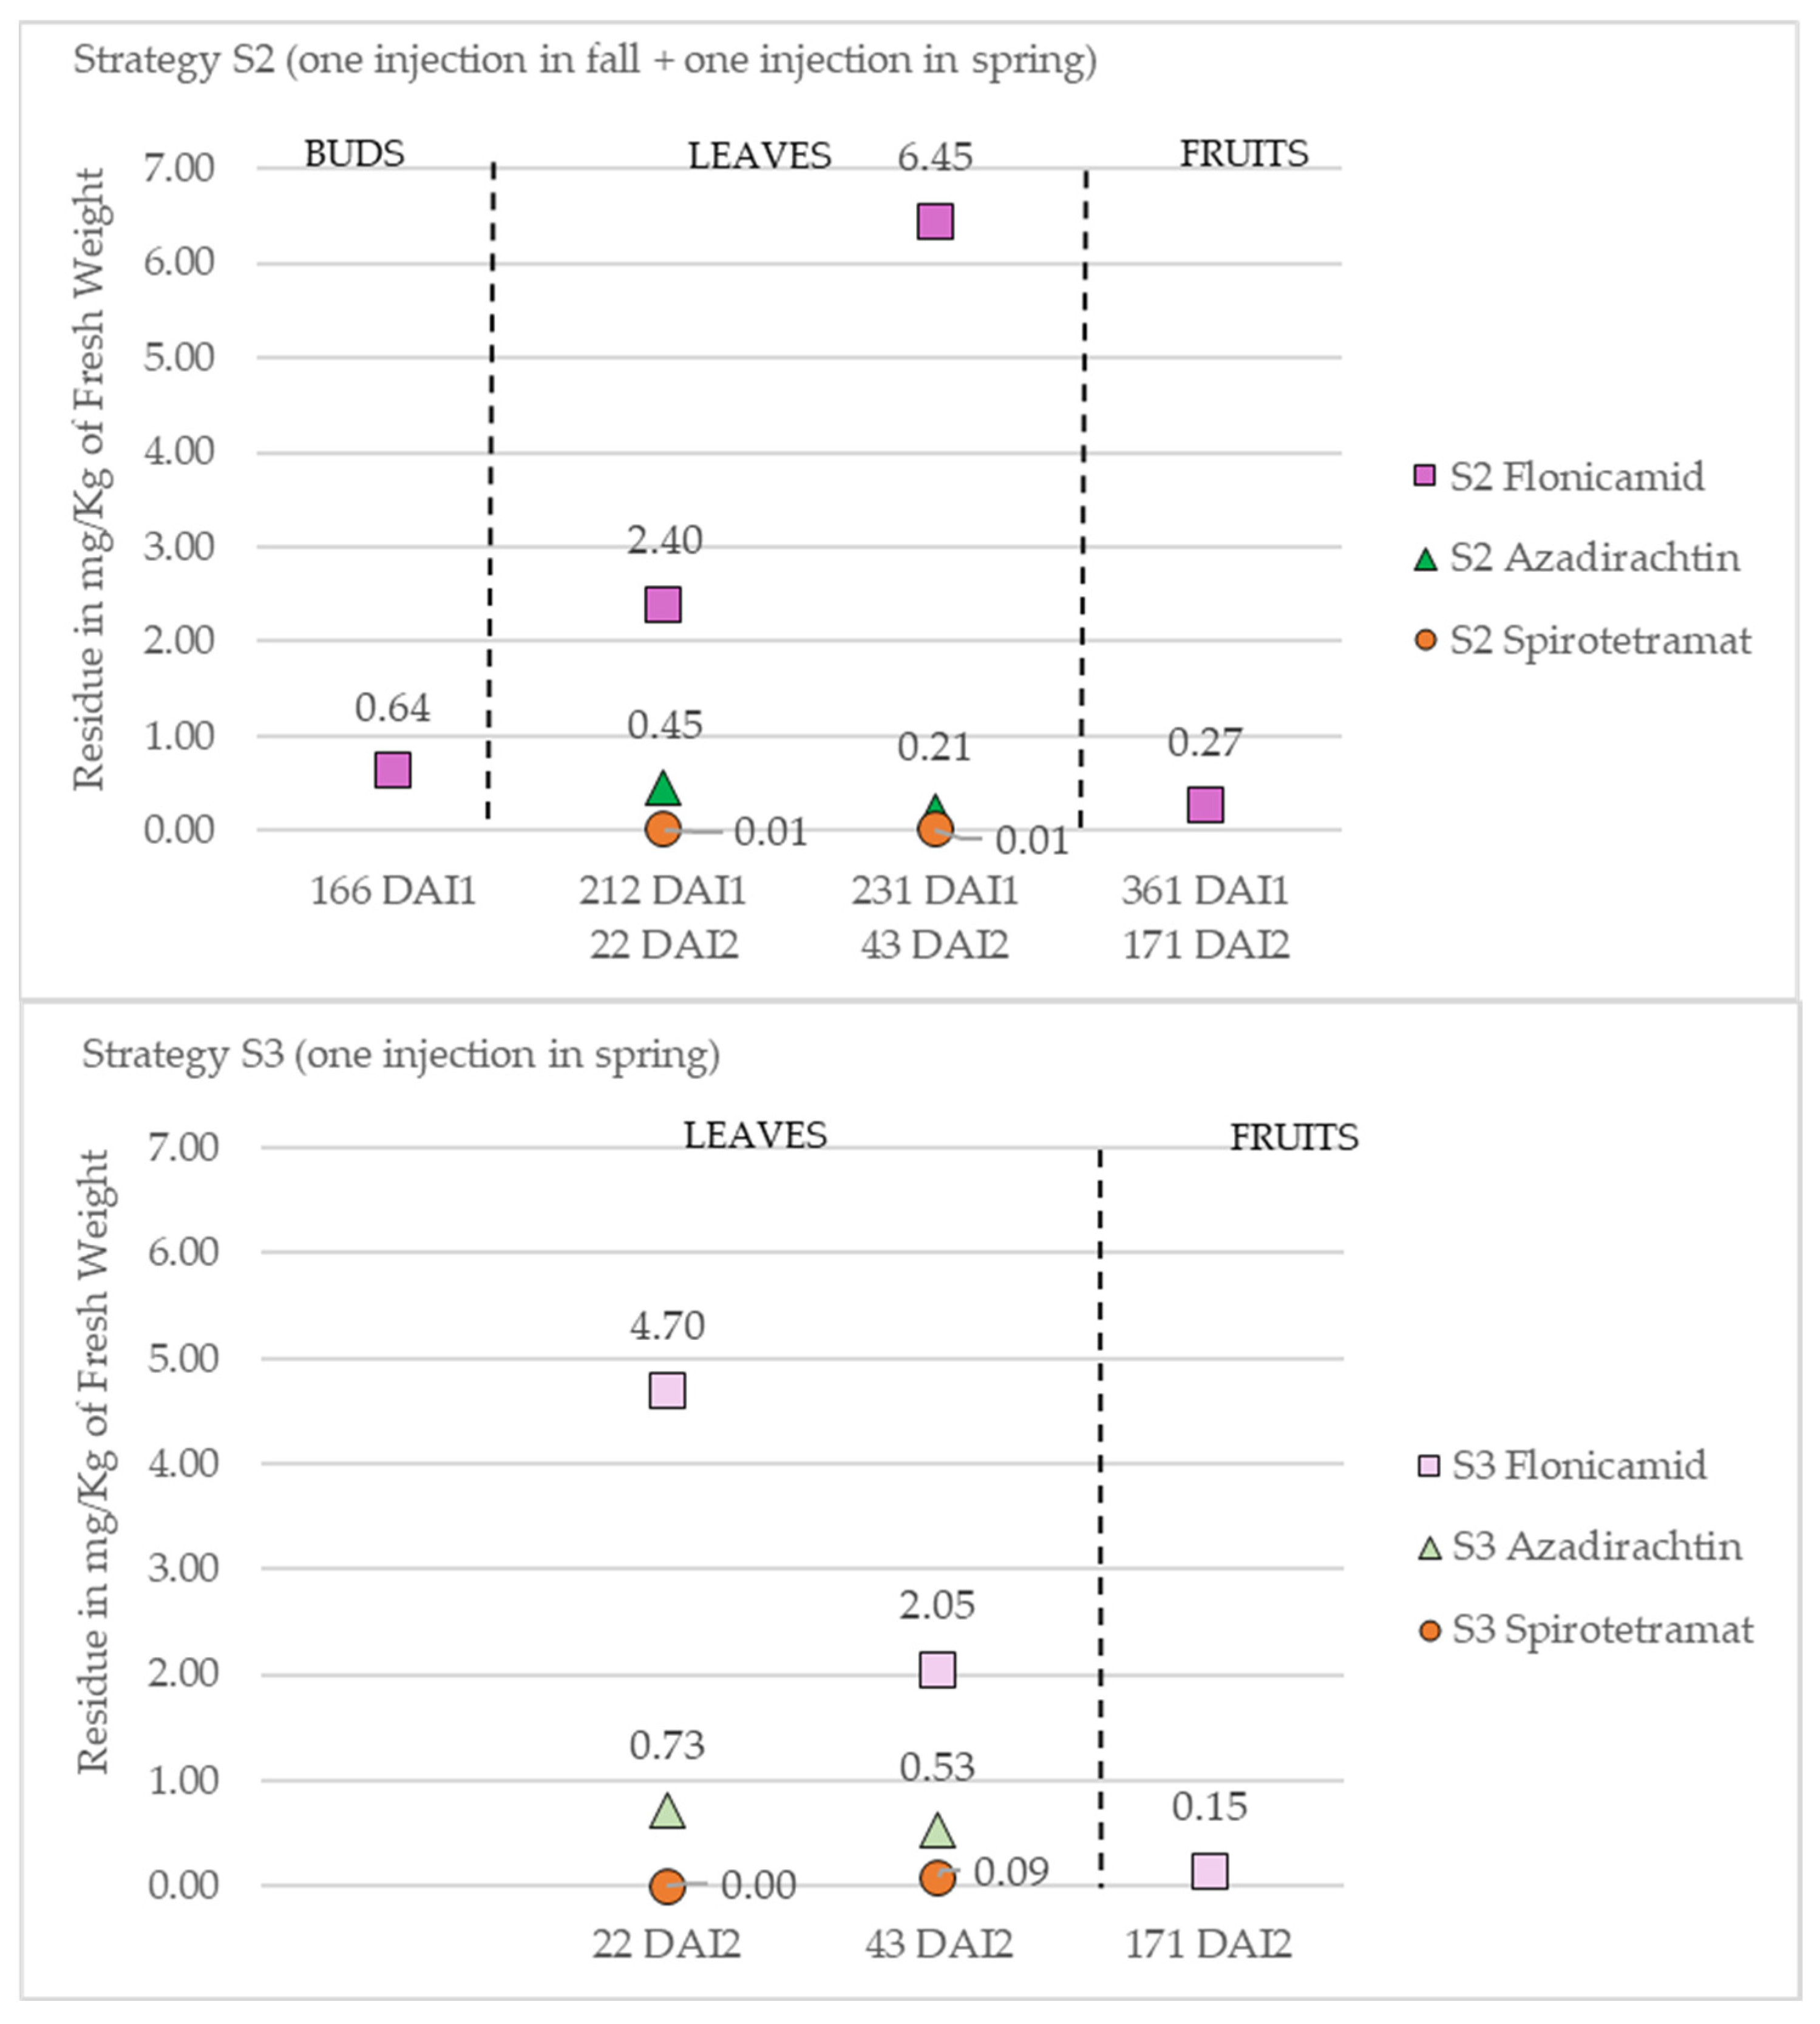
In 2023, samples in strategies S2 and S3 were taken from various organs: buds at the end of winter (27 February 2023), leaves on 12 April 2023 and 3 May 2023 followed by fruit samples at harvest time on 8 September 2023. These sampling dates were converted into days after injection DAI (
Table 3). Samples were frozen at −18 °C immediately after collection and then sent to the Eurofins laboratory (Eurofins Analytics France SAS, Nantes, France) for residue analysis. For all results, the amount of active ingredients detected in the samples was expressed in mg per Kg of fresh product.
2.6. Statistical Analysis
Statistical analyses were conducted in R Version 4.4.1. Prior to analysis, data were checked for assumptions of normality and homogeneity of variance. If the preceding conditions were met, an analysis of variance (ANOVA) was then performed. Where differences were significant (p < 0.05), post-hoc comparison of means was calculated using Tukey’s significant difference p-value adjustment for multiple pairwise comparisons. If the preceding conditions were not met, the data were transformed into log10(X + 1). If the normality and homogeneity of variance conditions were still not met, a non-parametric Kruskal-Wallis test was applied. Where differences were significant (p < 0.05), Dunn’s post-hoc test was used.
4. Discussion
The present study on the rosy apple aphid
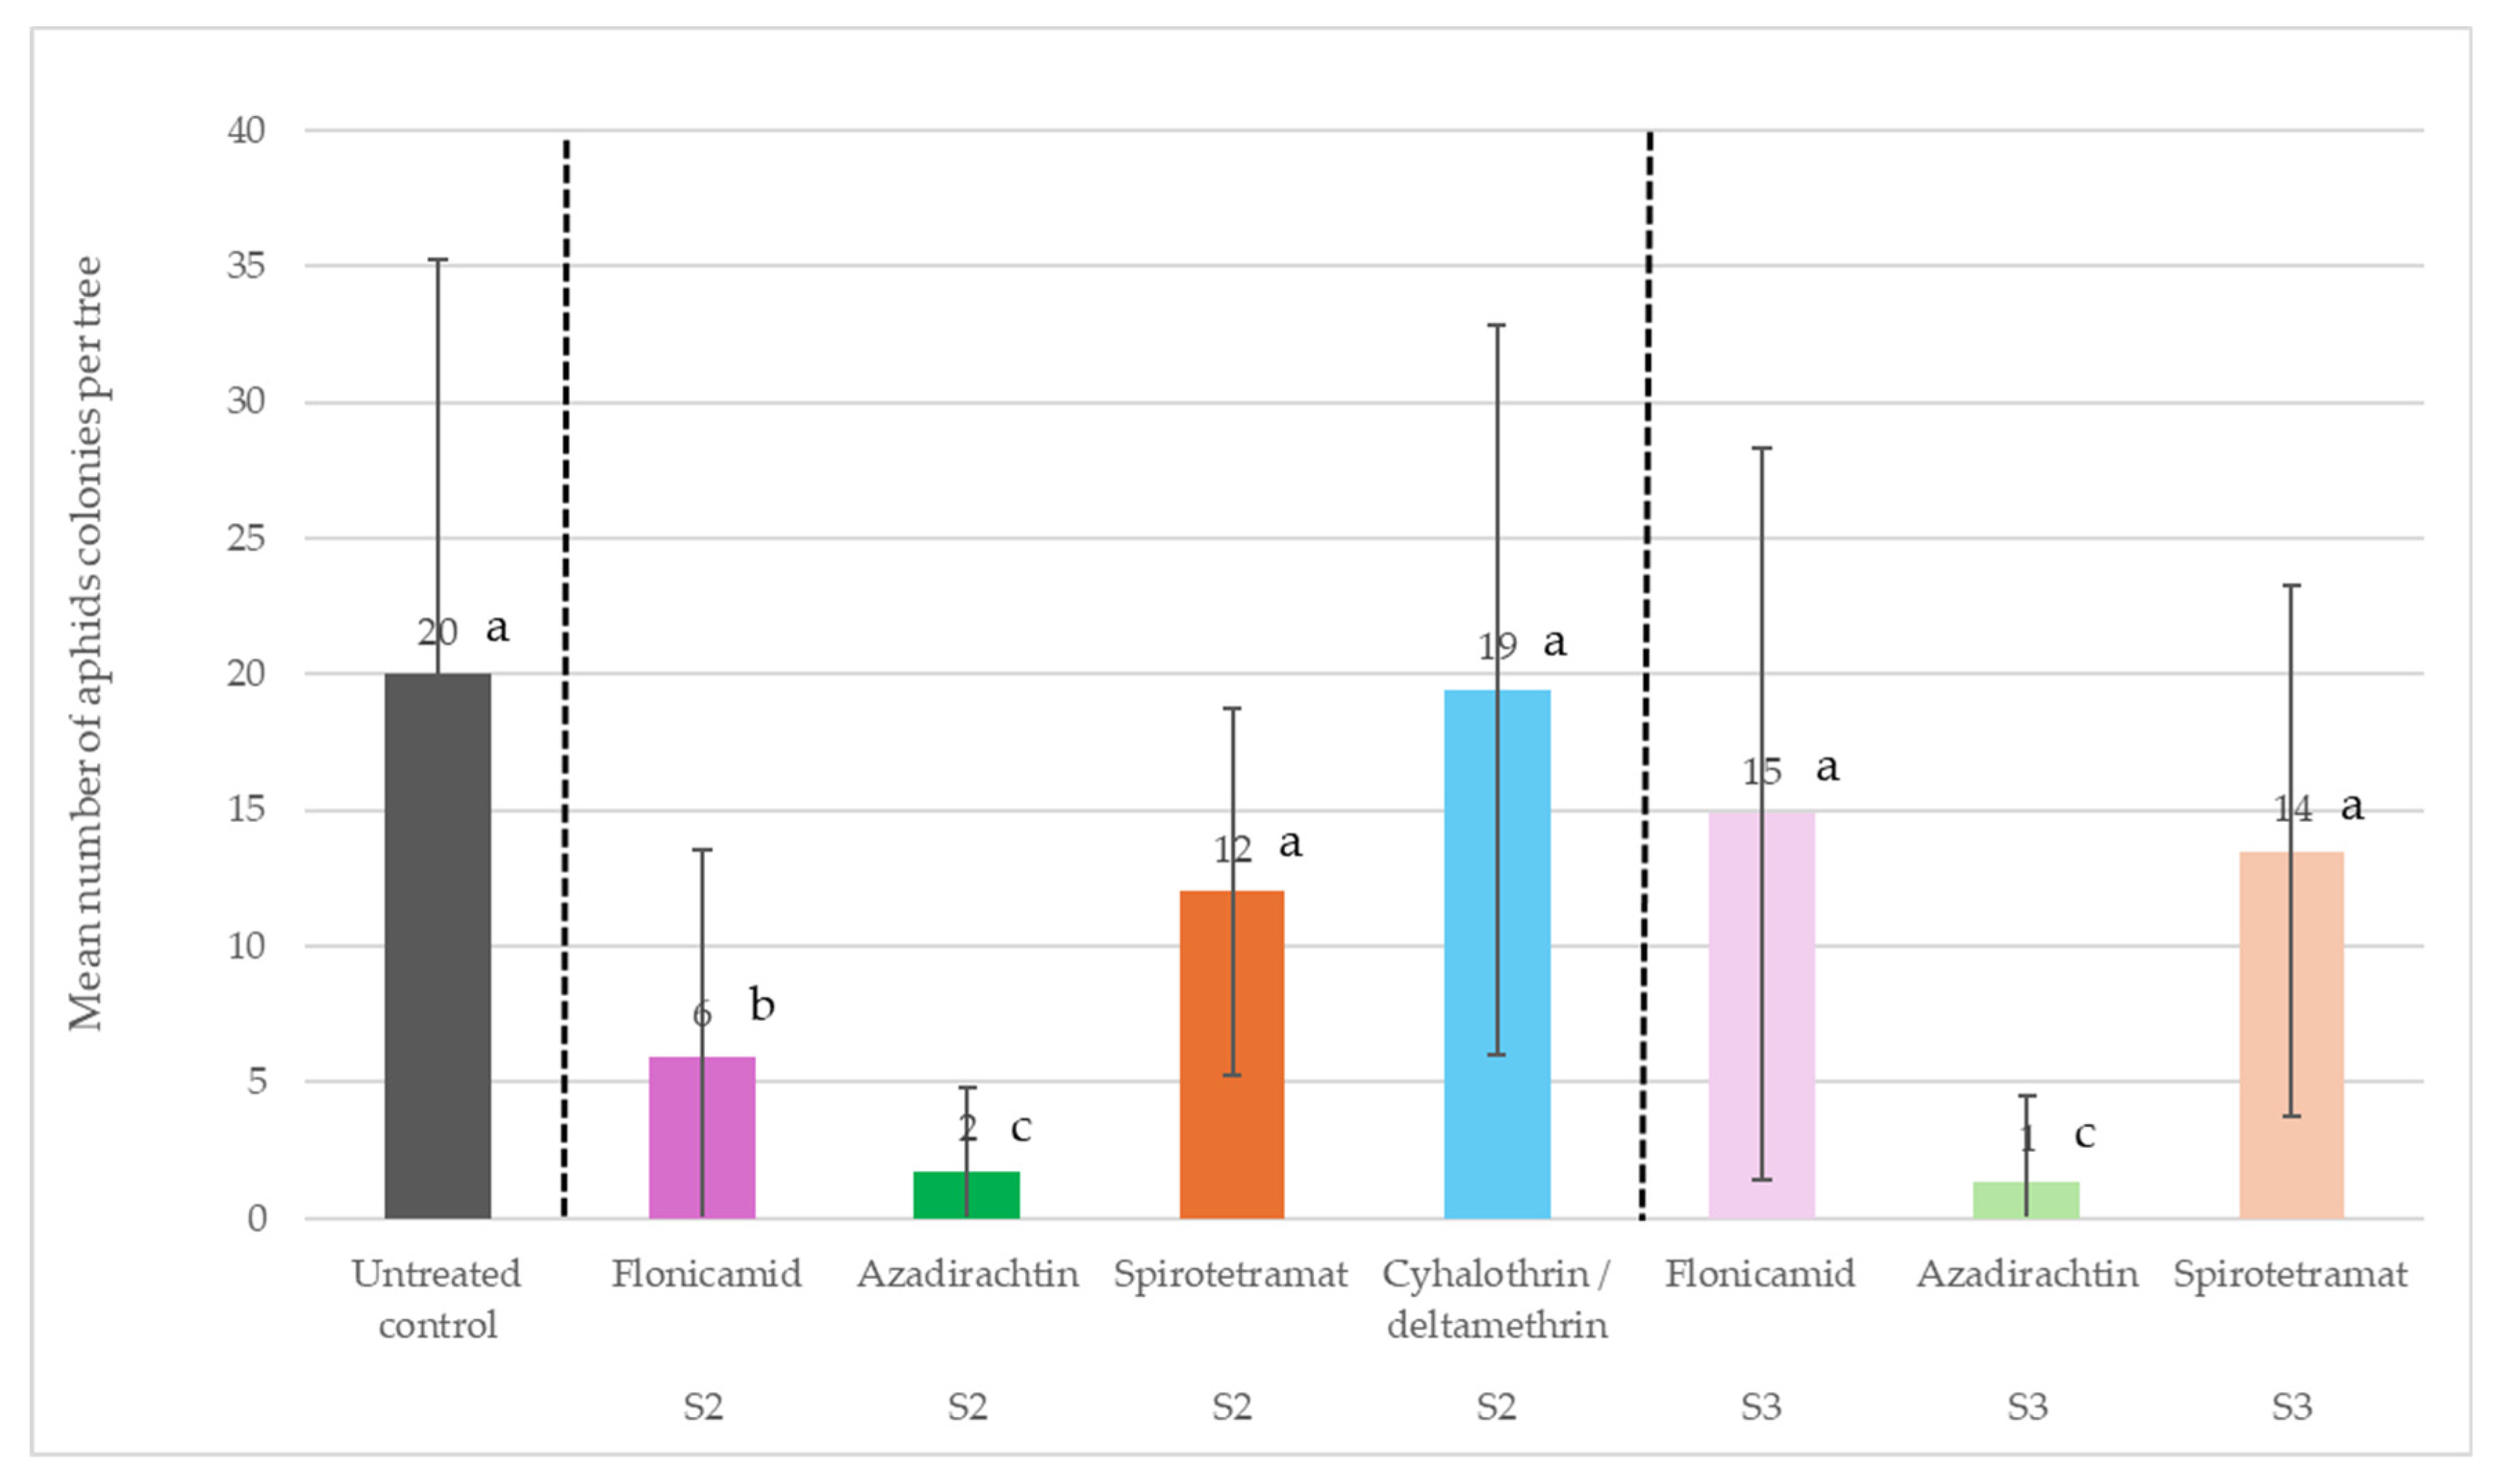
Dysaphis plantaginea highlights the potential of trunk microinjection as a viable alternative to traditional canopy spraying within increasingly stringent regulatory and societal frameworks. Notably, a single injection of azadirachtin achieved over 90% efficacy comparable to six to eight conventional spraying treatments required to manage this pest in the production area of South West of France. This level of control is particularly significant given the high pest pressure recorded during the 2023 and 2024 seasons. More broadly, these results demonstrate that trunk microinjection can achieve biological performance comparable to spray programs while drastically reducing the number of applications, confirming recent findings on the growing interest in trunk injection as a tool to reduce pesticide emissions and operator exposure in perennial crops [
21].
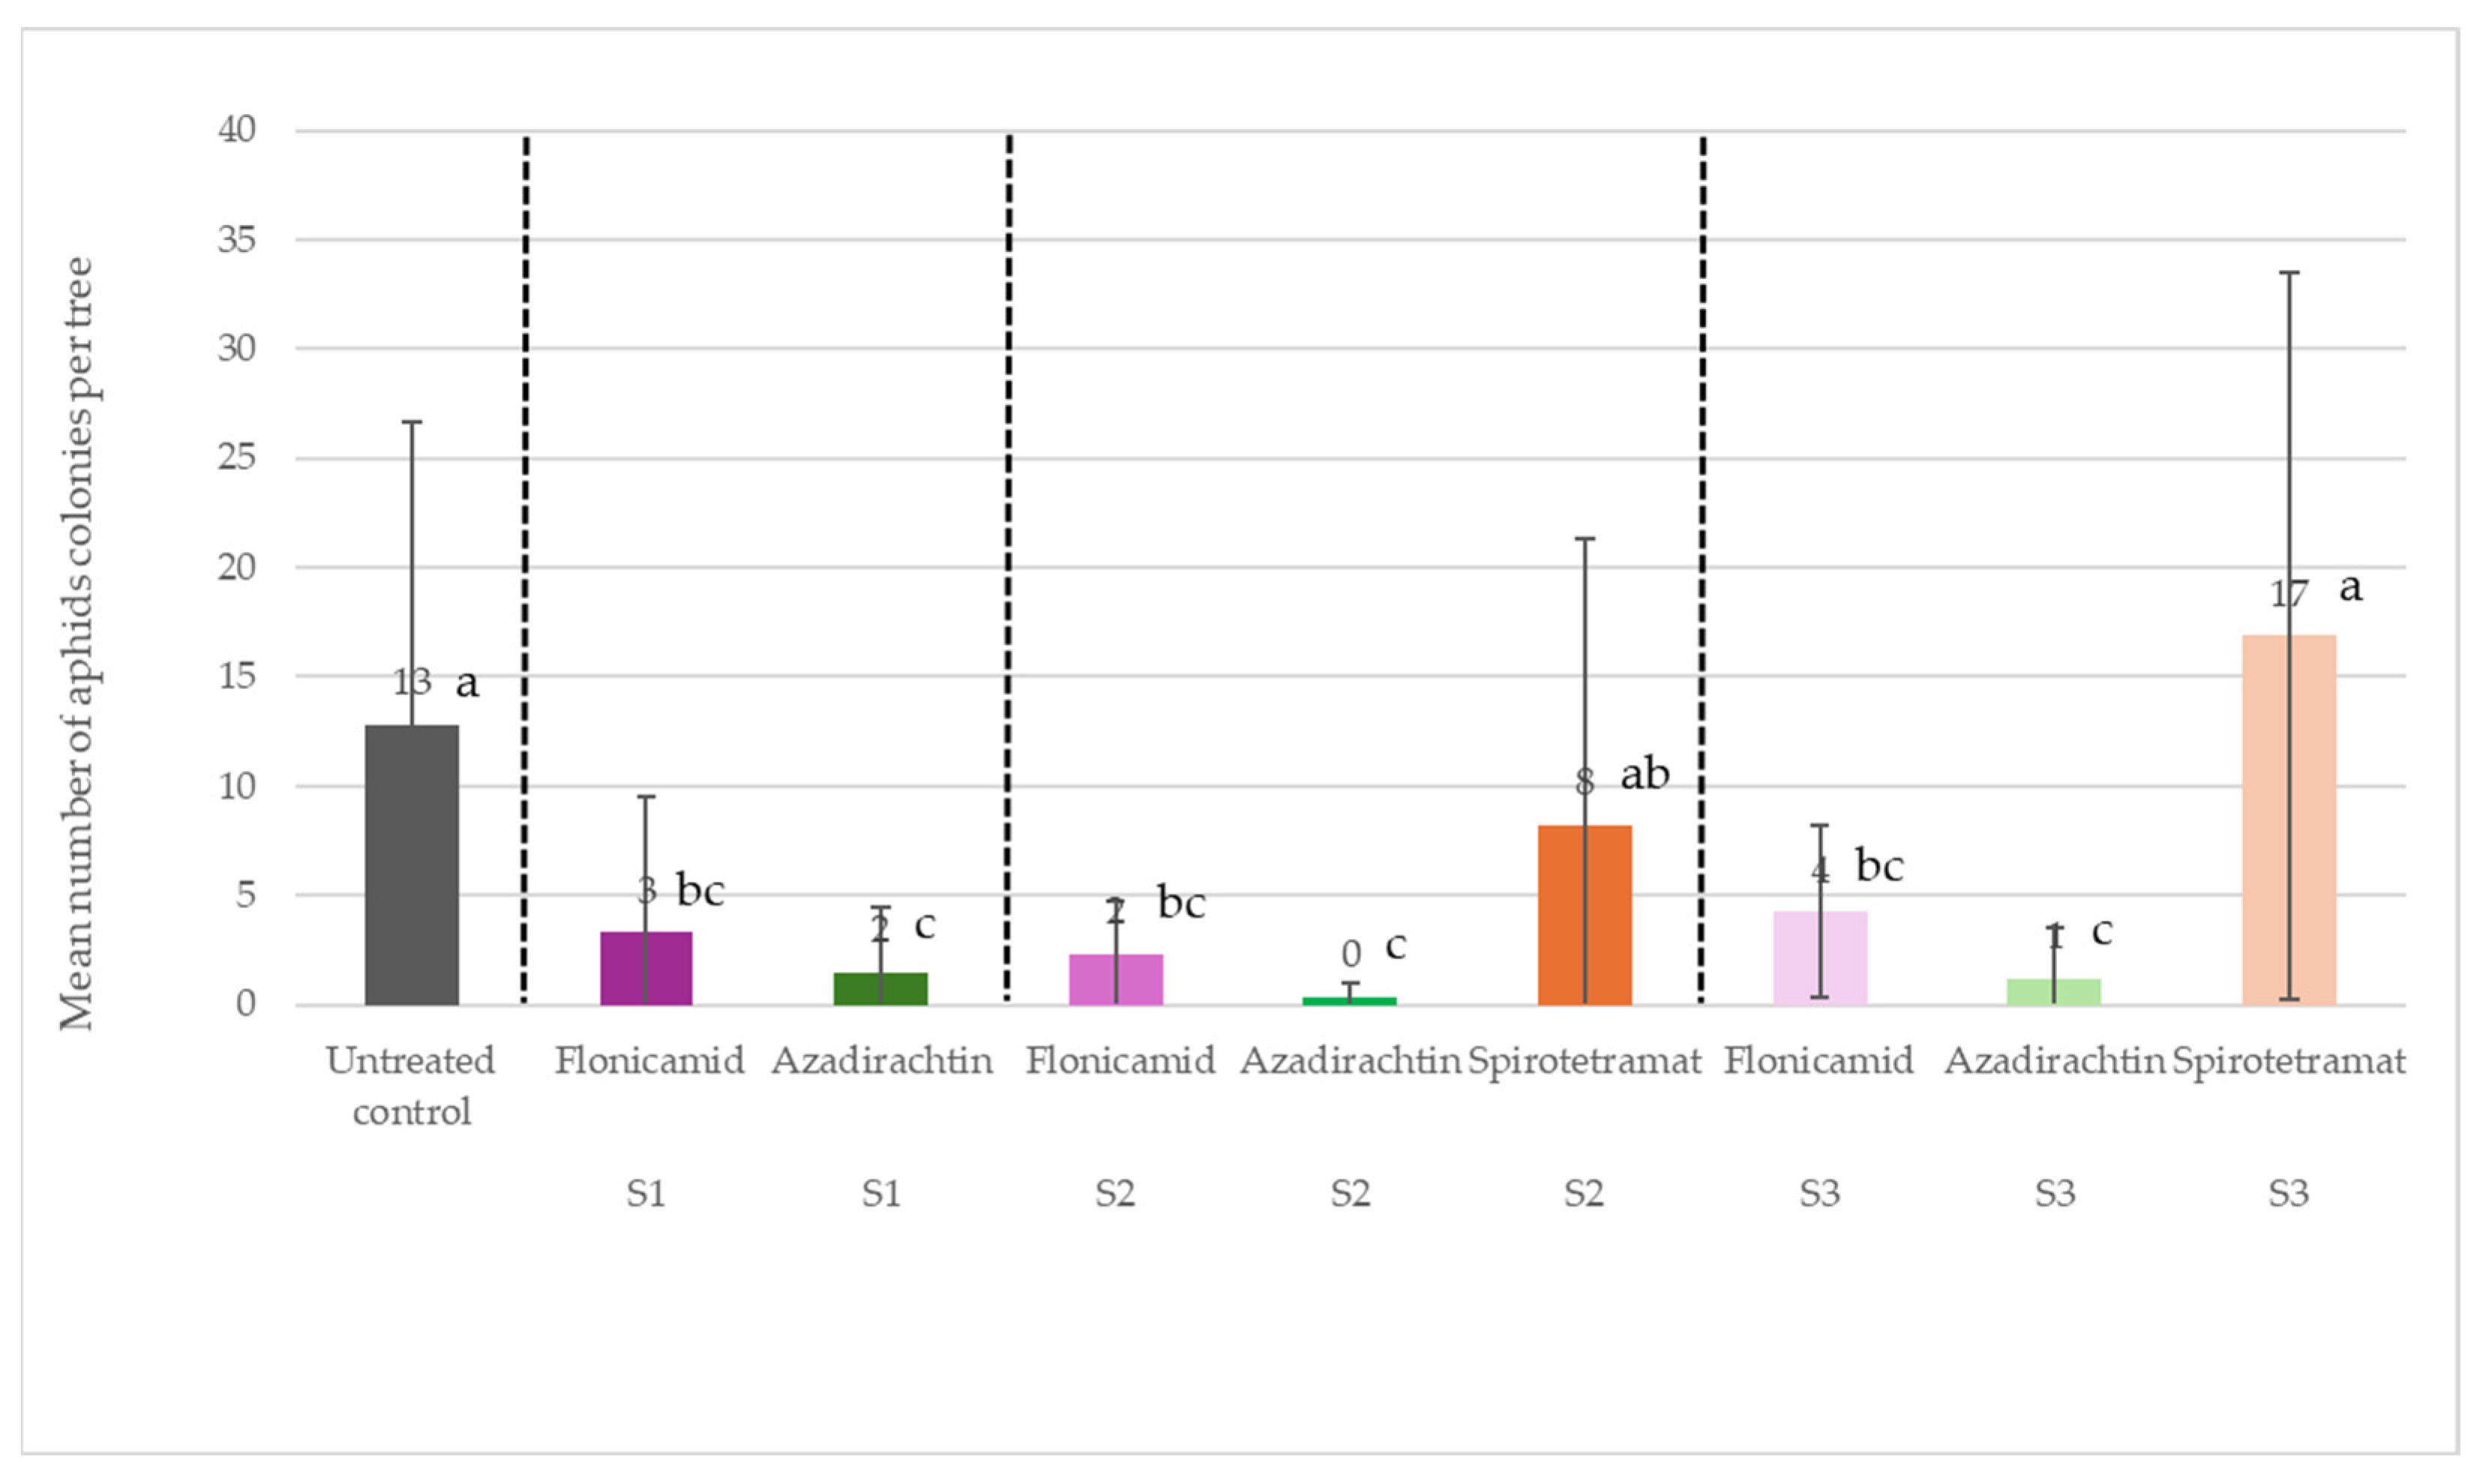
The results revealed a clear hierarchy in the efficacy of the injected compounds. Azadirachtin (as NEEMAZAL) emerged as the most consistent candidate, reducing fall infestation from 87 to 100% and post-flowering populations from 88 to 97%. Flonicamid (as TEPPEKI) demonstrated promising results with more variability. In contrast, spirotetramat (as MOVENTO) and the two pyrethroids tested (lambda-cyhalothrin and deltamethrin) showed highly variable and insufficient efficacy in terms of population control. This hierarchy is consistent with the theoretical framework based on xylem transport processes and highlights the central role of physicochemical properties in determining the success of trunk microinjection [
1]. The success of microinjection depends on four critical factors: (1) the migration of the product within the tree; (2) its uniform distribution within the tree; (3) the temporal synchronization with the target pest; and (4) the effective dosage required to reach the target pest. Among this, the ability of the active substance to move within the transpiration stream appears to be a key determinant. Compounds with low to moderate octanol–water partition coefficients (log K
ow) such as azadirachtin (1.09) and flonicamid (0.3) are more likely to remain in the aqueous phase of the xylem sap and be efficiently translocated toward actively transpiring organs such as developing shoots and leaves. This is supported by previous studies showing that systemic movement of injected compounds is closely linked to their physicochemical properties and plant transpiration dynamics [
1,
15].
In our study, the ideal candidate that meets all these conditions was azadirachtin. A single injection of this active ingredient provided highly effective control of
Dysaphis plantaginea throughout its entire life cycle. For comparison, in 2023 and 2024, the reference plot treated with a sprayer received seven applications of insecticides, to achieve an equivalent population control. The high efficacy of azadirachtin (as NEEMAZAL) may be explained by a combination of factors. First, its formulation (emulsifiable concentrate) likely promoted homogeneous dilution and efficient transport within the sap. Second, its physicochemical properties (moderate hydrophilicity, log K
ow = 1.09) favored upward migration. Third, azadirachtin has multiple modes of action. Research into the insecticidal effects of azadirachtin, a limonoid from the Indian Neem tree, Azadirachta indica, has been ongoing for some 30 years. Its strong antifeedant, insect growth regulatory and reproductive effects are now well understood and documented [
22]. This multi-target activity allowed it to affect several stages of rosy apple aphid life cycle, which is consistent with previous description of its biological activity on sap-feeding insects. In our study, the product injected in the fall was ingested by the wingless females present at that time, impacting their reproduction and thus the number of eggs laid before winter. Similarly, azadirachtin injected in the spring probably had a strong impact on the feeding and molting of the young larvae present in the spring. In our context, no significant differences were observed among the azadirachtin application strategies. Efficacy levels were comparable whether the product was injected in autumn, in spring, or in both autumn and spring. Few studies have addressed the trunk injection of azadirachtin in orchard systems; however, research conducted between 2017 and 2020 on the management of
Xylosandrus germanus (Coleoptera: Curculionidae) in topworked apple trees [
23] reported that spring injections of azadirachtin were more effective than autumn applications. Injection in spring coincides with a period of more intense flush and thus a greater abundance of new and rapidly transpiring leaves, which could allow for greater distribution of injected active ingredient in leaf tissue after the spring injection compared to after the fall injection [
11]. This theoretical principle could not be verified for azadirachtin in our experiment.
The second candidate to stand out was flonicamid, which showed good efficacy but with greater variability. Similar to azadirachtin, flonicamid has a low log K
ow (0.3), suggesting good mobility in xylem sap. Residue analyses confirmed its presence in plant tissues during rosy apple aphids’ activity period. However, despite promising efficacy (up to 89% efficacy in spring 2024), its performance was less consistent. This variability may be explained by formulation characteristics, as flonicamid was applied as a solid formulation requiring dissolution, which resulted in less predictable solubilization and transport. In addition, its dynamics within plant tissues may have been influenced by the physiological state of the tree, including transpiration rate and growth stage, factors already identified as key drivers of trunk injection performance [
15]. The observed variability may also be explained by the mode of action of flonicamid, which works only by disrupting the insects’ feeding behavior. Under our experimental conditions, observations made in 2023 highlighted differences among application strategies. Higher efficacy was achieved with two injections (one in autumn and one in spring) compared with a single spring injection which resulted in inconsistent results. However, this significant effect was not confirmed in 2024, when similar efficacy levels were observed regardless of the timing or number of injections.
Despite its favorable systemic profile a priori, spirotetramat did not demonstrate sufficient efficacy compared to the reference treatment. The very low residue levels detected in leaves suggested limited availability in target tissues. With a log K
ow of 2.51, spirotetramat is near the threshold above which mobility may be reduced, and partial adsorption onto xylem components cannot be excluded. Furthermore, spirotetramat requires metabolic conversion into its active enol form within the plant, a process that may limit its effectiveness when delivered exclusively through xylem transport. Similar limitations related to compound transformation and mobility have been reported in systemic insecticide studies [
2]. This lack of efficacy of spirotetramat applied via trunk microinjection is consistent with the findings of the only referenced study in fruit crops on trunk injection of spirotetramat (Movento) for the management of
Xylotrechus chinensis (Coleoptera: Cerambycidae) in mulberries [
24]. In this study, spirotetramat was the least effective insecticide against
Xylotrechus chinensis, with a performance almost equal to untreated trees.
Finally, the lack of efficacy of lambda-cyhalothrin and deltamethrin can be explained by their high lipophilicity (log K
ow values of 7 and 6.2, respectively), which prevented their transport in the aqueous xylem sap. Adsorption onto lignified tissues may strongly limit their mobility, resulting in negligible concentrations in aerial organs. Such behavior has been described for highly lipophilic compounds in woody plants, where strong binding to vascular tissues reduces bioavailability [
14].
Beyond active substance properties, since the tested formulations were not registered for trunk injection and were intended for spray application, formulation characteristics appear to be a critical determinant of injection success. Liquid formulations are likely to facilitate homogeneous distribution and transport within the sap flow, whereas solid or highly viscous formulations may lead to inconsistent delivery. This point is increasingly recognized in recent research, which highlights the need for formulation redesign specifically tailored to trunk injection systems, including improved solubility, stability, and compatibility with plant vascular tissues.
Another important factor is the temporal synchronization between compound availability in plant tissues and pest phenology. The results clearly show that autumn injections can reduce egg-laying by returning females, while spring applications target emerging populations. This confirms the importance of aligning treatment timing with pest life cycles, a key principle in integrated pest management strategies [
18].
Residue dynamics also provide valuable insights. Flonicamid showed higher and more persistent residue levels in leaves, indicating strong accumulation potential. However, this did not always translate into higher efficacy, suggesting that biological activity and mode of action are as important as concentration. Conversely, azadirachtin showed high efficacy despite lower residue levels, indicating strong biological activity even at low concentrations.
From an agronomic perspective, trunk microinjection offers major advantages. The drastic reduction in application frequency reduces labor, fuel consumption, and environmental contamination through spray drift, a major concern highlighted in previous studies on pesticide emissions [
3,
4]. In addition, individual tree treatment opens new possibilities for precision crop protection strategies. However, several limitations remain, including variability linked to tree physiology, operational constraints for large-scale orchards, and the need for specific regulatory frameworks adapted to injection-based delivery systems.
Overall, these findings demonstrated that trunk microinjection has strong potential as a sustainable plant protection strategy in orchards, provided that suitable active ingredients and formulations are selected and that application timing is optimized in relation to both plant physiology and pest dynamics.