


Abstract
As the population ages, the incidence of age-related neurodegenerative diseases is rapidly increasing, and novel approaches to mitigate this soaring prevalence are sorely needed. Recent studies have highlighted the importance of gut microbial homeostasis and its impact on brain functions, commonly referred to as the gut–brain axis, in maintaining overall health and wellbeing. Nonetheless, the mechanisms by which this system acts remains poorly defined. In this review, we will explore how (poly)phenols, a class of natural compounds found in many plant-based foods and beverages, can modulate the gut–brain axis, and thereby promote neural health. While evidence indicates a beneficial role of (poly)phenol consumption as part of a balanced diet, human studies are scarce and mechanistic insight is still lacking. In this regard, we make the case that dietary (poly)phenols should be further explored to establish their therapeutic efficacy on brain health through modulation of the gut–brain axis, with much greater emphasis on carefully designed human interventions.
1. Introduction
An increase in the average age of the population is closely correlated with a similar increase in age-related diseases, including those affecting the brain [1]. A staggering 152.8 million cases of dementia are expected worldwide by 2050, having detrimental effects on individuals, their families, and the global economy [2,3]. Consequently, it is vital to understand how to support brain health and to develop strategies to delay cognitive decline during ageing, improving the quality of life of individuals, and addressing a major public health challenge.
The dynamic, bi-directional communication between the gut and the brain, also known as the “gut–brain axis” (GBA) has been the centre of extensive research in recent years. The GBA refers to the communication between the brain and the gut microbiota via multiple different pathways, as reported by us and others [4,5,6,7,8,9]. In addition, the functioning of the nervous system is affected by both the immune and the metabolic state of the body, with the gastrointestinal tract (GI) playing a major modulatory role [10,11].
The human GI tract is a rich and diverse ecosystem enabling several important physiological roles such as the maintenance of the host immune system and the integrity of the gut barrier through the production of various endogenous metabolites. For example, the gut microbiota may produce metabolites directly from the food ingested (e.g., short chain fatty acids; SCFAs), modify host-related metabolites (e.g., secondary bile acids), or produce de novo metabolites (e.g., polysaccharide) [12,13]. Indeed, the metabolism of different food components provides a wide range of by-products that can directly positively or negatively affect host health [14]. Moreover, the metabolic state of the organism also impacts the production of gut-derived metabolites, mainly through varying substrate availability, intestinal transit time [15] or redox balance [16], ultimately contributing to the overall homeostasis of the organism [17,18].
Dietary plant-derived (poly)phenols are an integral part of the human diet and can modulate the composition of the gut microbial community [17,19]. This interaction between gut microbes and metabolites of food-derived compounds appears to positively impact on human chronic diseases [20,21] and be a highly relevant modifier of brain physiopathology [22,23]. Consequently, research in the field of the GBA is now investigating how the gut microbiota can be a target for nutritional and therapeutic strategies to improve brain health during ageing. This review will explore the impact of (poly)phenols on the gut–brain axis and their potential role in promoting overall brain health.
2. The Microbiota–Gut–Brain Axis and Ageing
The mounting interest in the gut microbiota and its role as a contributing factor in health and disease has highlighted its potential impact on various pathologies, including neurodegenerative diseases. The gut microbiota is a concentrated population of 1010 to 1011 microbes per wet-weight gram of faeces [24], although it may be underestimated due to the presence of other microbes in the intestinal mucosa and other faecal fluids [25]. It is comprised of bacteria, archaea, fungi, and viruses, interacting with their host, affecting many important functions such as nutrient metabolism, xenobiotic and drug metabolism, maintenance of structural integrity of the gut barrier, immunomodulation, and protection against pathogens [26]. Its composition is highly variable, although a number of key bacterial species are typically present in most individuals. Several factors influence this variability, with the type of birth (vaginal vs. caesarean section) to diet being the most impactful [27,28,29]. An imbalance in microbial community structure, sometimes termed as gut dysbiosis (almost wrongly, as the healthy/eubiotic microbiome is not yet defined) or the lack of colonisation resistance (resilience to the invasion of pathogens) [30] can encourage the growth of pathobionts which will compete for nutrients, modify metabolite production or enhance immune responses [31]. Pathogenic bacteria can cause inflammation by altering the gut environment and exploit compounds derived from the commensal microbes for their own growth. Increased intestinal permeability, enabling diffusion of pathogenic bacteria into the systemic circulation and ultimately the brain, may lead to synaptic dysfunction and neuronal loss, eventually affecting cognitive and memory function [32]. Taken together, these processes may contribute to pathological brain ageing and eventually Alzheimer’s disease (AD) [33].
2.1. The Gut Microbiome and Ageing
The impact of the microbial composition and associated changes suggests that microbes can accelerate the ageing process [34]. Biological vulnerability and decreased physiological reserves associated with neurobiological changes such those observed in age-related frailty [35], collocate with a reduction in gut microbiome diversity in the elderly [36,37]. Research has highlighted a distinct change in the gut microbiome profile of centenarians, characterised by a rearrangement of the Firmicutes population and an enrichment in facultative anaerobes, including potential pathobionts [38]. This change in microbial composition may have a negative impact on the host, particularly due to the under-representation of species known to produce SCFAs such as butyrate, which are essential for stimulating epithelial cell growth and promoting gastrointestinal health [39]. Studies have also explored the association between specific age-related traits, such as frailty, and the functional profile of the gut microbiome in rodents [40]. Findings reveal that ageing may be associated with changes in taxonomic and functional patterns, including the under-maintenance of specific host nutrition-related functions [41,42]. More recently, increasing microbiome compositional uniqueness was shown to both reflect healthy ageing and predict lifespan in older adults [43]. This increase in uniqueness is accompanied by a decline in the core genus Bacteroides, marking it as a characteristic of healthy ageing. Furthermore, studies of faecal microbiome repository data across five continents and with participant ages ranging from 18 to 107 years old showed that gut microbiome alterations associated with both typical and pathological ageing are likely characterised by a loss of the stable components of the microbiome and concomitant increase in disease-associated taxa [44] (Figure 1).
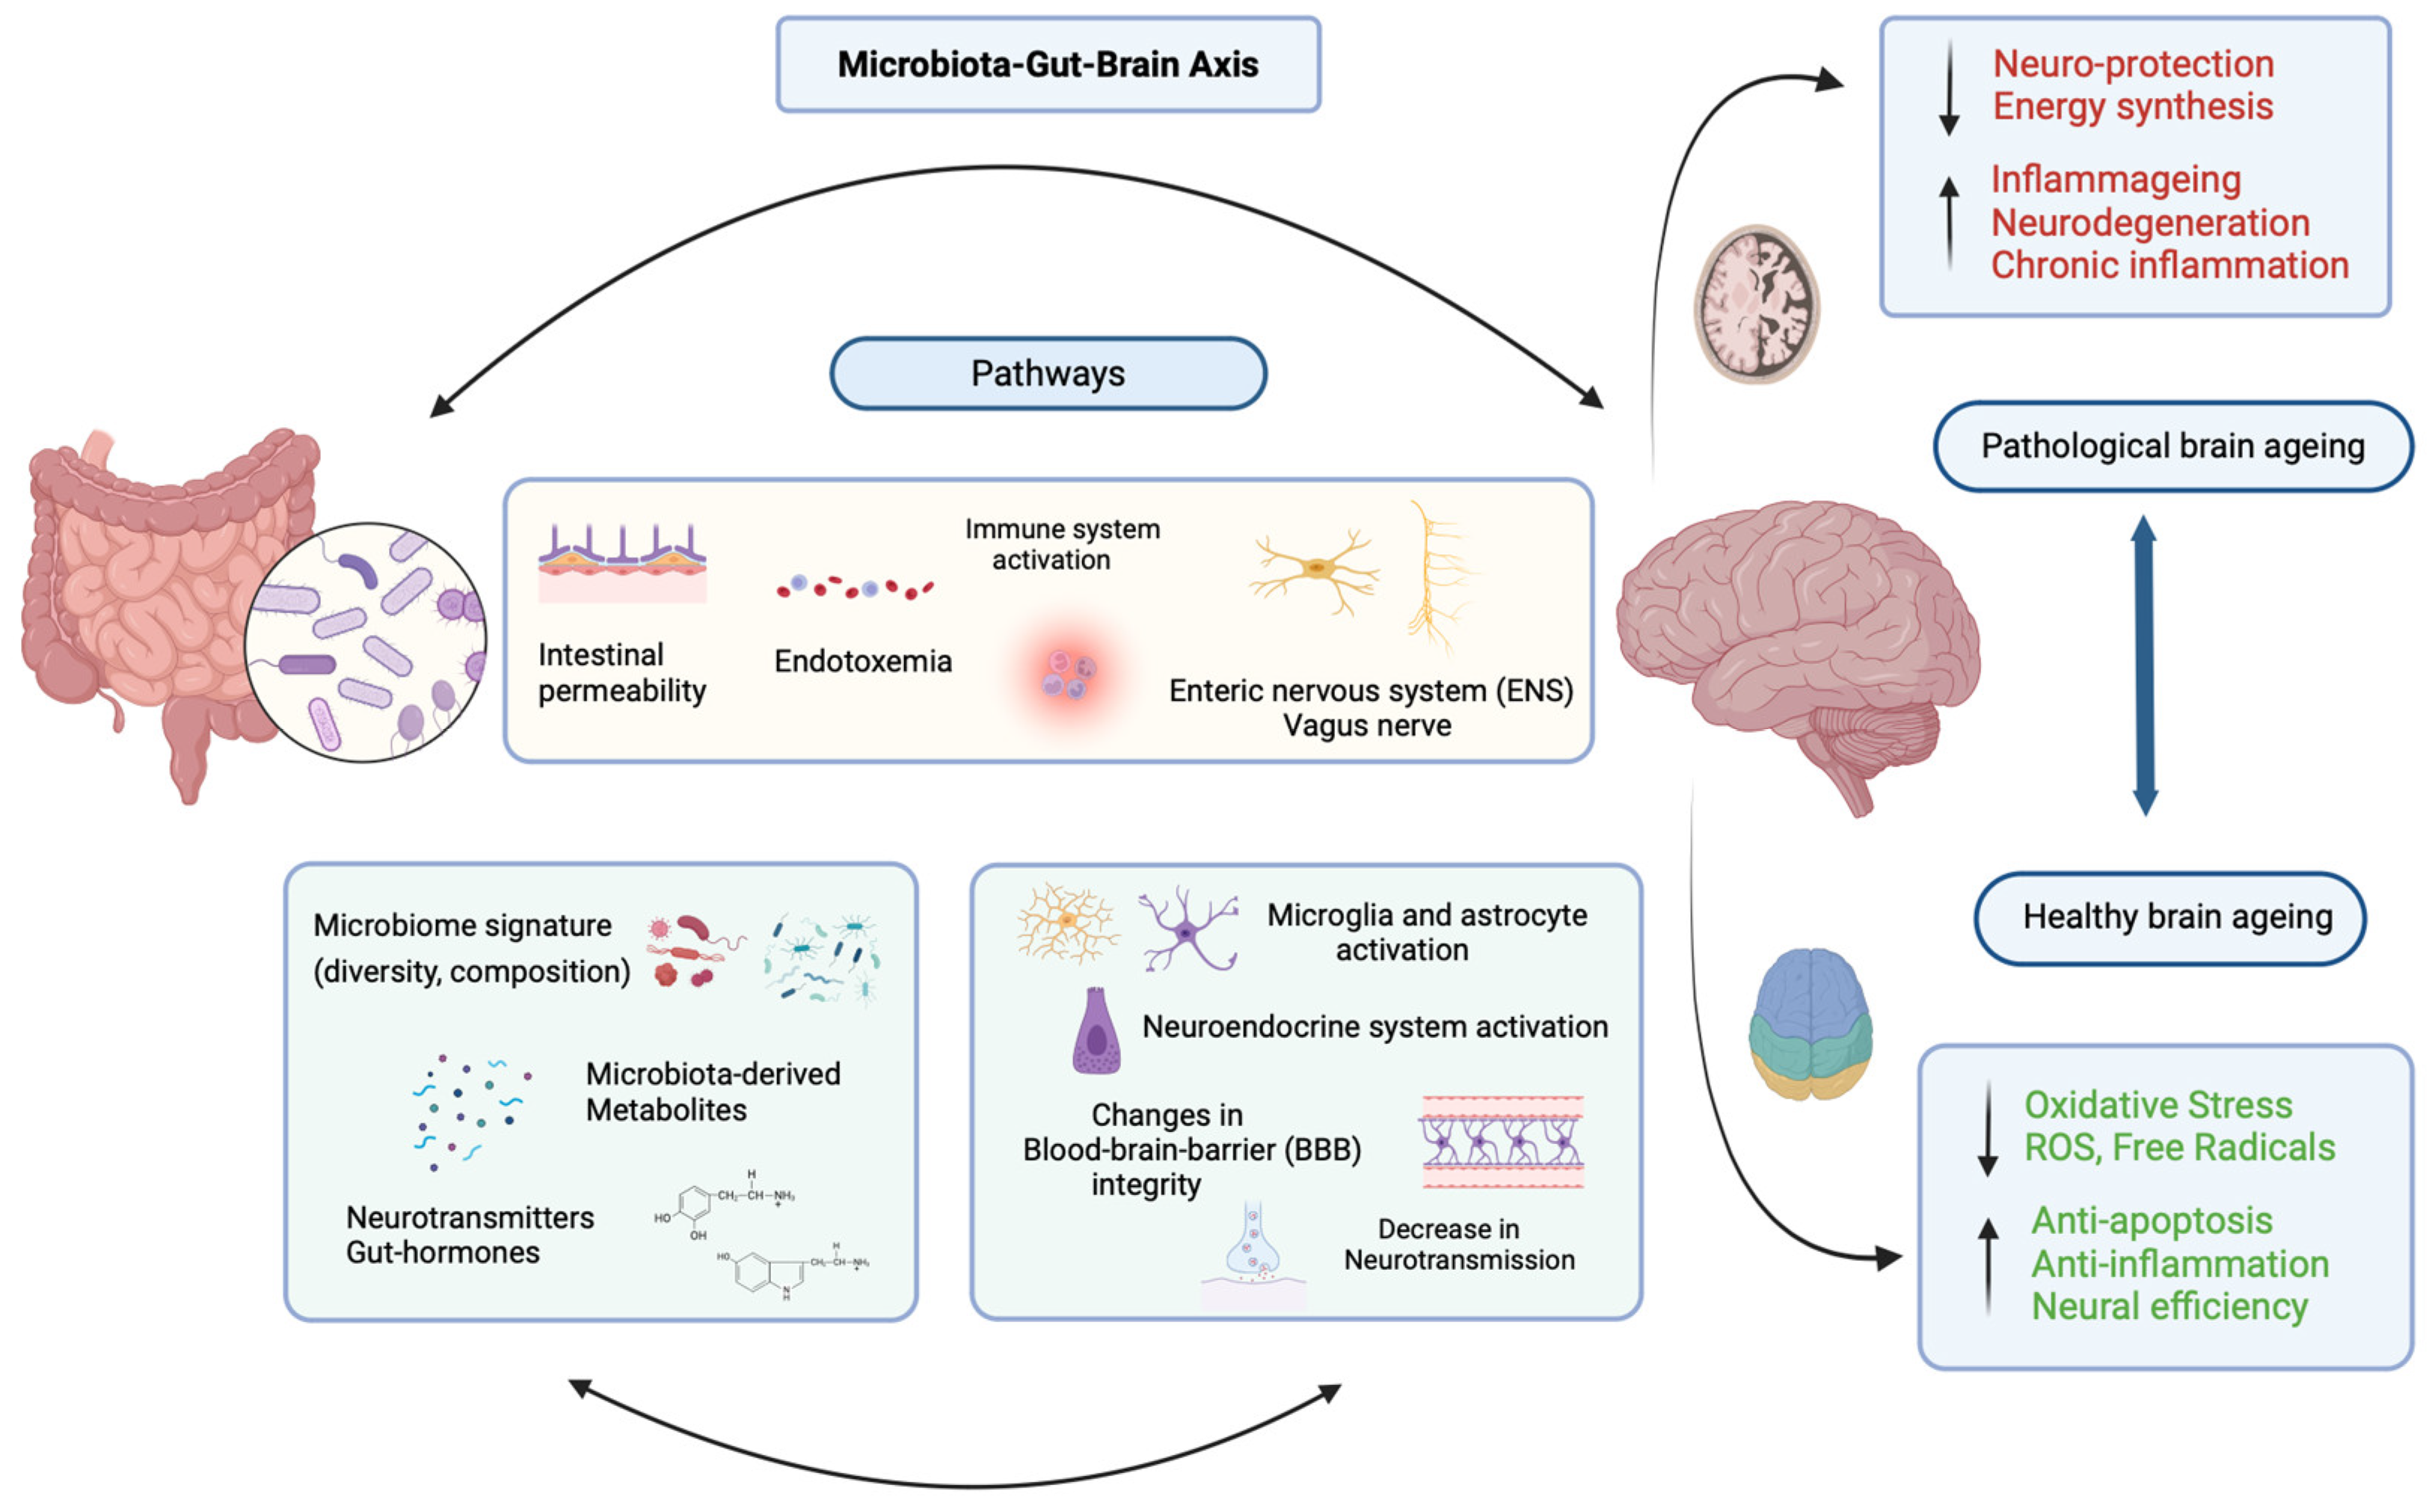
Figure 1.
The microbiome gut–brain axis and its importance in modulating brain health during ageing. Overview of pathways through which the gut microbiota interacts with the brain, the factors influencing microbiome composition, and the resulting effects on brain health. The gut microbiome can influence intestinal permeability and modify gut barrier integrity. Increased gut permeability can lead to the presence of endotoxin in the blood stream (endotoxemia), activate the immune system and influence systemic immune responses. Direct communication channels between the gut and the brain are occurring for example via the Enteric Nervous System (ENS) and the vagus nerve among others. The composition of the gut microbiota can influence neurotransmitters and gut hormones levels, as well as the levels of gut-derived neuroprotective metabolites, and impact signalling pathways involved in cognitive functions and neuroactivity. Dysregulation of the microbiota–gut–brain axis can lead to neuroprotection deficits, reduction in energy synthesis and neurodegeneration (microglia and astrocyte activation), all characteristics of a pathological brain. On the other hand, proper functioning of the gut–brain axis can counteract oxidative stress, reduce reactive oxygen species (ROS) and free radicals, promote anti-apoptotic mechanisms, enhance anti-inflammatory responses, and improve neural efficiency, thus supporting a healthy brain during ageing (created with BioRender.com (https://biorender.com/, accessed on 21 April 2024).
2.2. Gut Microbiota, Inflammation, and the Blood-Brain Barrier
One of the body’s natural defence systems to fight external stressors is inflammation. Although beneficial in the short term, persistent low-grade inflammation may fuel the development of neurodegenerative diseases and is accompanied by a parallel systemic immune dysfunction [45]. Low-grade chronic inflammation, also termed ‘inflammageing’, is promoted by both endogenous and exogenous triggers, with the gut microbiota now recognised as a key player [46]. Controlling, slowing or reversing low-grade inflammation is likely to be an important approach to prevent or minimise the severity of age-related functional decline, including in the brain, and the onset of conditions which adversely affect health and well-being. In addition to inflammation, central to brain health is the control of influx and efflux of biological substances essential for brain metabolism and neuronal function, processes ensured by the blood-brain barrier (BBB) [45]. The main role of the BBB is to protect the brain from toxic substances in the blood and to act as a filter for nutrients [47], but when its integrity is damaged, it is thought to permit and contribute to neuropathological processes. Pathogenic bacteria can invade the brain through a variety of complex putative mechanisms [48], a feature that may be affected by gut microbial changes. Homeostasis of the gut microbiome can ensure better gut barrier integrity, thereby limiting bacteraemia, systemic inflammation and ultimately potential brain invasion by pathogens. The absence of a commensal microbiota certainly influences BBB development, disrupting expression of the tight junction proteins crucial for optimal BBB efficacy [49] (Figure 1). Interestingly, BBB disruption was partly restored following either colonisation of germ-free mice with a conventional murine microbiota or upon feeding with a sodium butyrate solution. Other gut-derived metabolites such as trimethylamine N-oxide (TMAO), p-cresol conjugates and propionate have also been reported to exert protective effect upon the BBB [50,51,52] which further complicate our understanding of the bacterial-host interactions in healthy and pathological ageing.
2.3. The Gut–Brain Axis and Neurological Disorders
The autonomic nervous system plays a significant role in gut–brain communication, with both the parasympathetic vagus nerve and multiple sympathetic efferent fibres connecting and regulating endocrine, immune, humoral, and gastrointestinal functions. The vagus nerve represents a particularly important link between nutrition and neurological and inflammatory diseases, with vagal activity having been shown to modulate the enteric nervous system (ENS) and the gastrointestinal tract, with the gut microbiota playing a mediatory role [53,54]. Notably, alterations in the ENS occur prior to CNS manifestations of pathology, suggesting a potential ‘‘anticipatory” pathological communication with the brain [55]. Moreover, the ENS can be potently influenced by gut microbes, such that disorders in the gut microbes can prime disorders in the ENS. Given that disturbances in the ENS correlate with disorders in the CNS, it is unsurprising to observe GI issues in diseases impacting the nervous system and neurological disorders [56]. Indeed, in some neurological diseases, particularly Parkinson’s disease, peristalsis is compromised resulting in constipation and GI symptoms occurring in 60 to 80% of patients [57,58,59].
2.4. Diet, Gut Microbiota, and Gut–Brain Communication
Diet plays an important role in gut–microbiota and gut–brain communication, but these interactions are complex and multi-faceted [60]. Indeed, diet composition and the gut microbiome regulate production of a broad range of metabolites [61], but the potential influence of these compounds on cognitive health are only beginning to be uncovered. For example, although short chain fatty acids, secondary bile acids, TMAO, tryptophan derivatives, cresols and other metabolites have been reported to affect cognitive function and neurodegenerative disorders [22,61], this represents only a small fraction of the known microbe-derived molecules in the circulation. Thus, the microbiota and diet are critical modulators of gut–brain communication (Figure 1).
3. (Poly)phenols, Gut–Microbiota–Brain Axis and Ageing
Plant-derived (poly)phenols, a group of naturally occurring phytochemicals present in high amounts in fruits, vegetables and cereals, in addition to their impact on brain functions [62], have been reported to impact the intestinal microbiota by supporting the proliferation of beneficial microbes or by suppressing the proliferation of pathogens [63]. Indeed, a “prebiotic-like” effect of phenolic compounds and (poly)phenol-derived gut microbial metabolites has been reported to increase protective strains of bacteria, to decrease pathogenic inflammatory microorganisms, and to influence the Firmicutes/Bacteroidetes ratio, that is altered with ageing [17,64]. However, the different biological activities of various (poly)phenols will depend both on their bioavailability, itself influenced by factors such as age, sex and body composition, and on their secondary metabolites produced by the gut microbes [60,61], potentially explaining inter-individual variability in response to (poly)phenol intake [65]. Evidence that interactions exist between (poly)phenols and brain health, mediated via effects on the gut microbiome and inflammatory pathways, is compelling and widely reported [66], but whether products of polyphenol-mediated gut microbial metabolism are associated with brain activity is far less well-established [67].
With the aim of capturing the current evidence of the role of (poly)phenols on the gut–brain axis and their impact on brain health, we conducted a non-systematic comprehensive literature search, using keywords related to brain health and cognitive status, polyphenolic compounds, gut microbiome composition and metabolites related to brain health. This search resulted in 462 hits up to 9 November 2023. Following a first screen based on title and abstract readings, the full text screening resulted in 56 studies (53 preclinical and 3 clinical) that were included in this review and are detailed below. The results retrieved are presented in the Table 1 for preclinical studies and in the Table 2 for clinical studies.
3.1. Preclinical Evidence
3.1.1. (Poly)phenols, Gut Microbiome Modulation and Related Brain Health
The significant role of (poly)phenols in modulating the gut microbiome and their potential benefits for brain health and cognitive functions is evident through various studies on flavanols, flavonols, flavones, phenolic compounds, polyphenol-rich extracts and other botanicals (Table 1). These studies have demonstrated that (poly)phenols such as epigallocatechin gallate (EGCG) and epicatechin (EC) can increase both bacterial and species richness, decrease harmful bacteria such as Proteobacteria, and increase the abundance of beneficial bacteria such as Akkermansia and Bifidobacterium [68]. The modulation of the gut microbiome is associated with decreased activation of the microglia and inflammatory pathways in the brain, suggesting a protective effect against neuroinflammation and cognitive decline. Similarly, flavonols (e.g., quercetin) have been reported to increase the abundance of beneficial gut bacteria, such as Barnesiella and Lactobacillus, while decreasing the detrimental taxa Alistipes and Rikenella (Bacteroidetes phylum) [69]. These changes in the gut microbiome are linked with improved spatial memory, decreased amyloid-beta (Aβ) accumulation, and tau phosphorylation in mice, indicating potential benefits for AD prevention. Phenolic compounds such as curcumin and sesamol have also been associated with alterations in gut microbiota composition, leading to improved spatial learning and memory, decreased Aβ pathology in the hippocampus, and reduced neuroinflammation [70,71,72] suggesting neuroprotective effects of these compounds. Moreover, other (poly)phenols including fisetin [73], icariin [74] and various flavones such as baicalein [75,76] and apigenin [77] have also been reported to improve behavioural impairments, enhance motor learning and coordination, and decrease neuroinflammation through modulation of the gut microbiota composition and microbial metabolites. (Poly)phenol-rich extracts and botanicals, such as blackberry and blueberry anthocyanin-rich extracts [78,79], have been shown to restore gut dysbiosis, increase the production of SCFAs, improve cognitive performance and improve antioxidant activities in the brain. Overall, (poly)phenols improve gut microbiome composition by increasing microbial abundance and diversity and by restoring a gut microbial balance between the Firmicutes/Bacteroidetes ratio [74,80,81,82].
3.1.2. Insight into Associated Molecular Mechanisms
The positive impact of (poly)phenols on the gut microbiome are in turn linked with improved cardiometabolic functions, reduced immune activation and secretion of anti-inflammatory molecules, and a tangible positive effect on the intestinal barrier. In particular, (poly)phenols modulate the expression/regulation of key genes/pathways related to antioxidant activities, maintenance of the BBB integrity, and overall brain functions, including the regulation of astrocytes and microglia activities. These beneficial changes are most often correlated with increased relative abundance of Bacteroides, Akkermansia, Lactobacillus, Lachnospiraceae, Ruminococcus, Muribaculaceae, and Bifidobacterium (Figure 2).
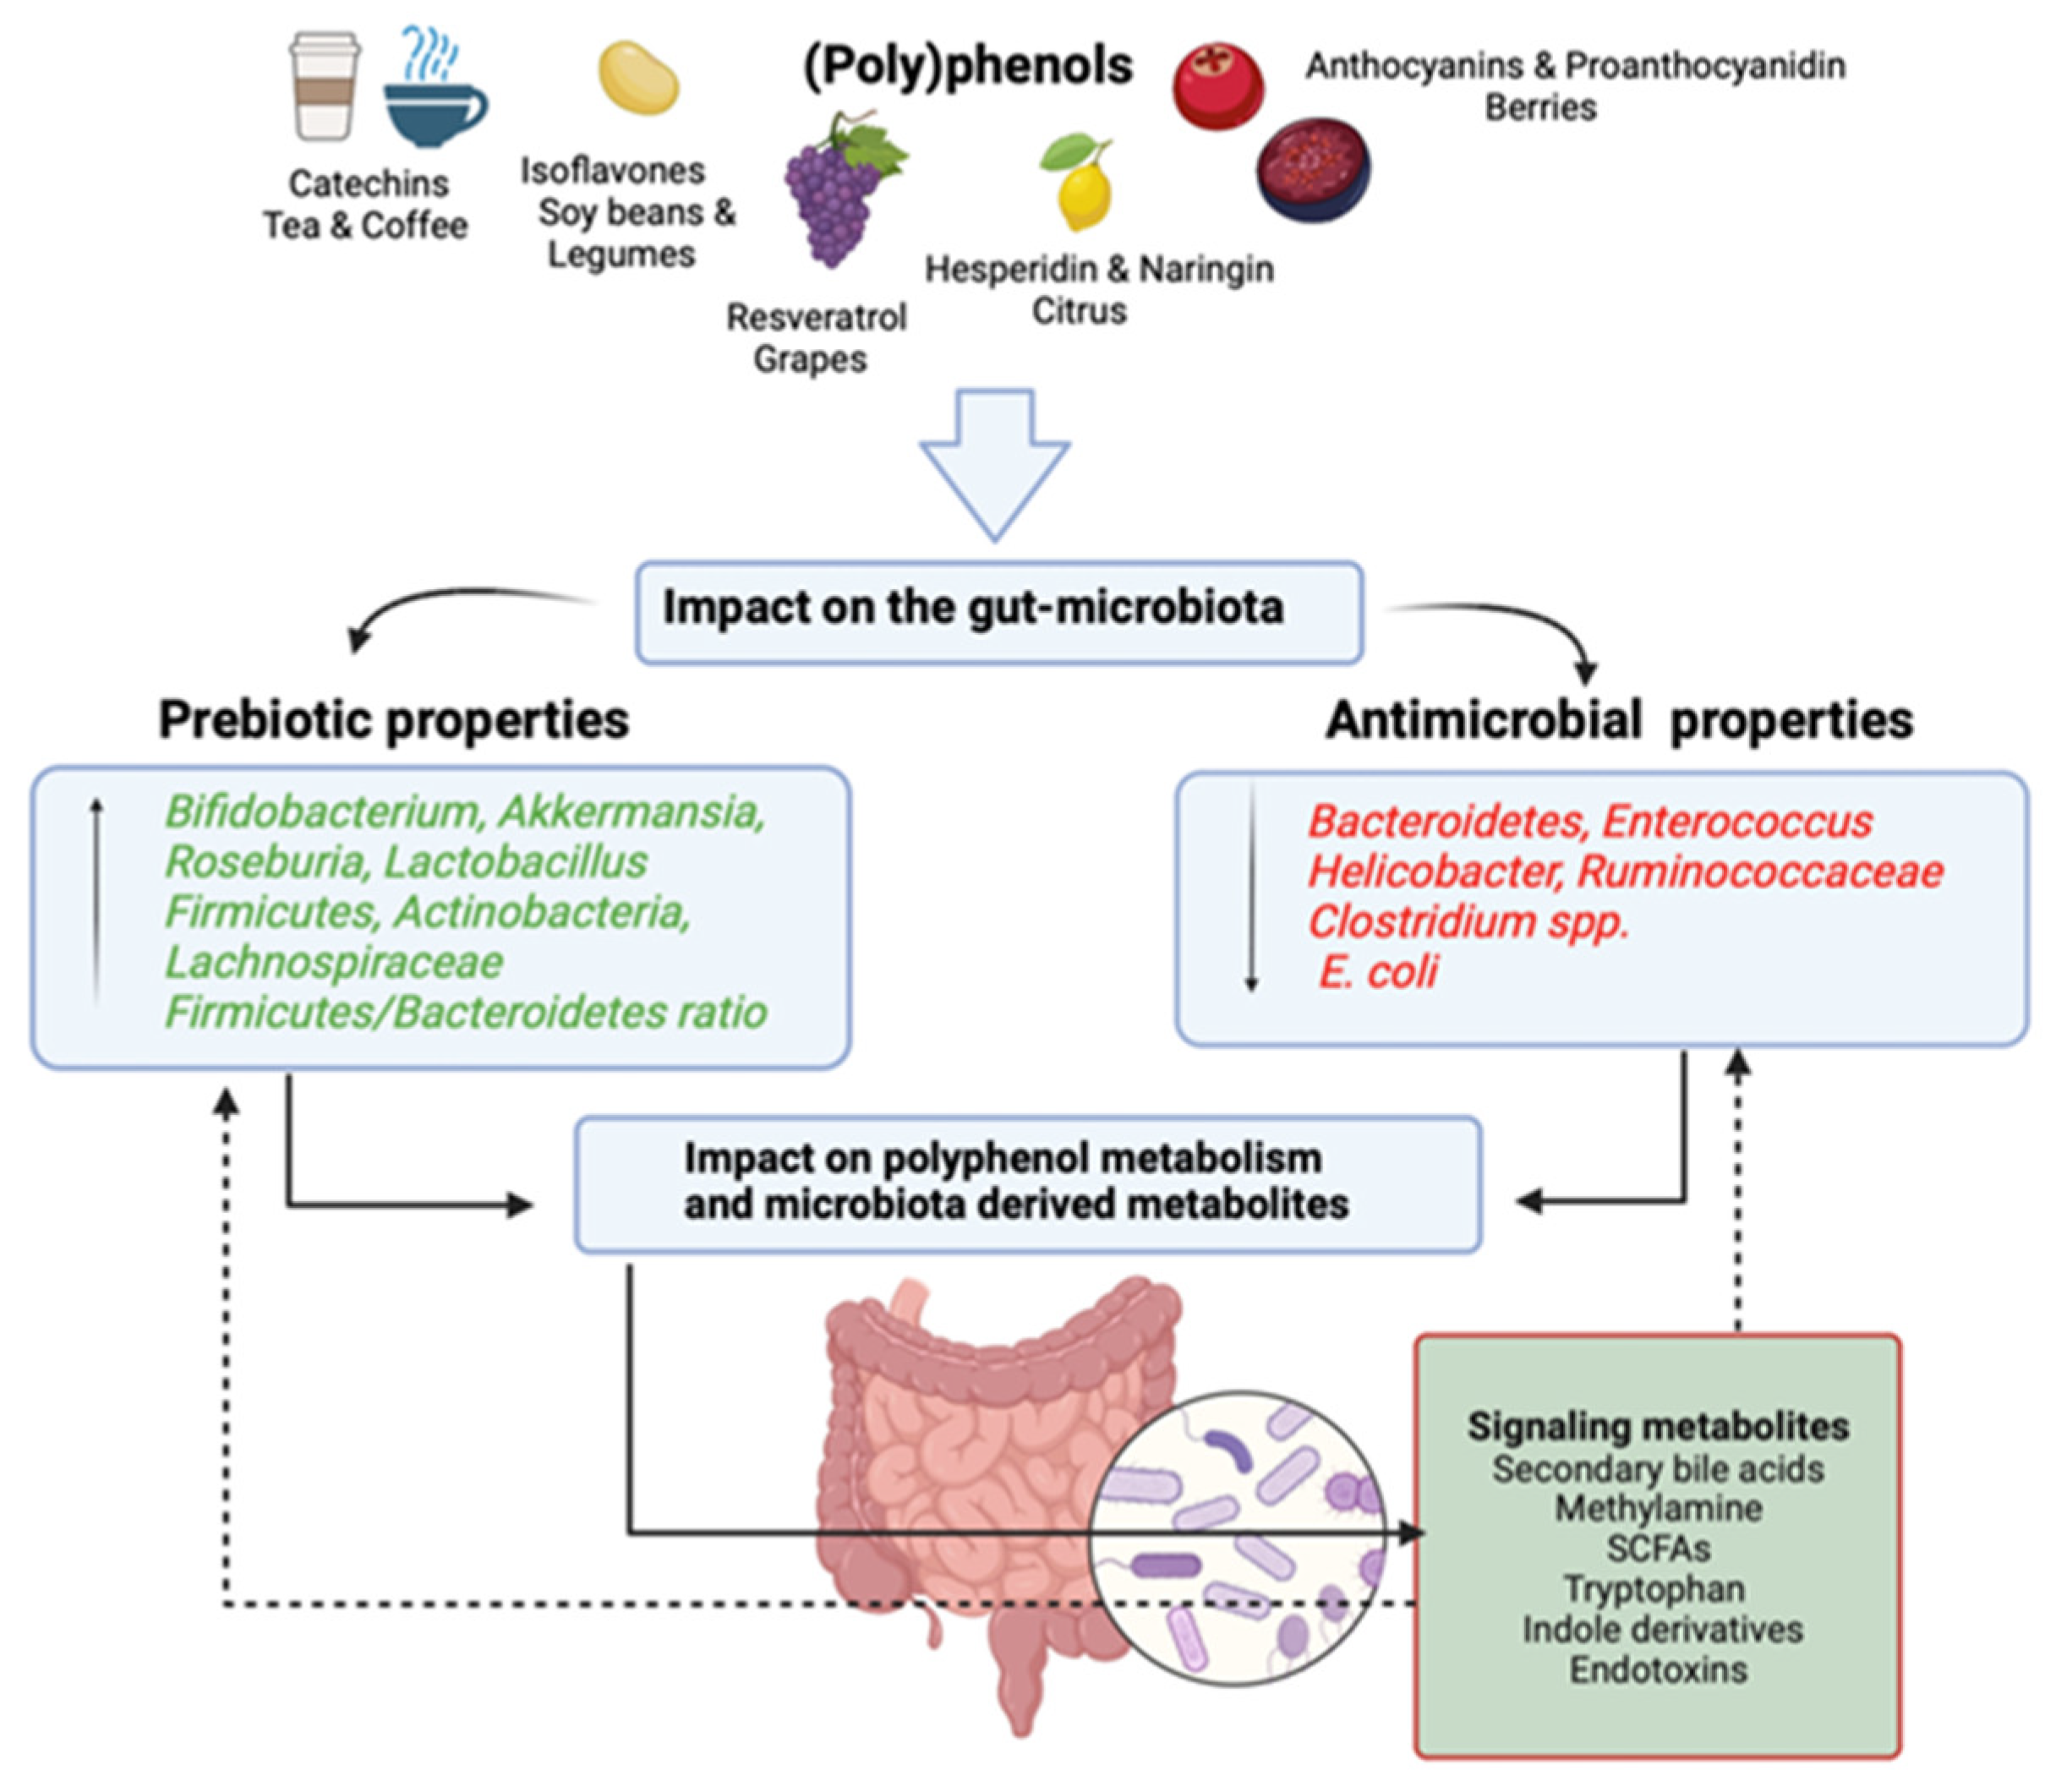
Figure 2.
Impact of (poly)phenols on gut microbiota. The activities of the diverse (poly)phenol sources and their impacts on the gut microbiota of which prebiotic and antimicrobial properties, polyphenol metabolism and microbial-derived metabolites influence the gut ecosystem (created with BioRender.com).
These observations include an increase in neurotrophic factors such as BDNF, a down-regulation of inflammatory pathways and a reduction in pro-inflammatory cytokines (IL-1β, IL-6, and TNF-α) and endotoxins (LPS). The effects of (poly)phenol on the gut microbiome and neurological health, including major disease-related aspects such as the reduction in pathological protein aggregation, the restoration of hippocampal neuronal plasticity or increased expression, which are key regulators of barrier integrity [77,83,84,85,86]. The interaction between (poly)phenols and LPS occurs in multiple ways, either by inhibiting the expression of pro-inflammatory cytokines and LPS-induced mediators [87], suppressing TLR4/NF-κB pathways [87,88], attenuating LPS-induced oxidative stress [89] or even by binding LPS directly, therefore preventing its interaction with cellular receptors [90]. However, the response to LPS is dose-dependent, and health effects vary according to its exposure. High levels of LPS can cause endotoxemia, leading to septic shock and severe human health consequences [91,92]. Consequently, the beneficial effects of (poly)phenols from this angle should be taken with reserve when assessing their effects, particularly under acute conditions.
In addition, reduction in oxidative stress mediated by improved antioxidant defence and increased enzymatic activity (e.g., superoxide dismutase (SOD) or catalase (CAT)) is also commonly reported in pre-clinical studies. Neuronal tissues have a high metabolic rate, and therefore produce elevated amounts of reactive oxygen species (ROS) when compared to other organs [93]. For example, during the mitochondrial oxidative phosphorylation, anion superoxide is generated as a by-product of ATP, and transformed into oxygen. Both commensal and pathogenic gut bacteria have the capacity to modulate mitochondrial activity, and therefore to alter ROS production [94]. In addition, metabolites such as SCFAs help to regulate redox homeostasis by influencing mitochondrial activity [95] via the induction of signalling pathways such as the nuclear erythroid 2-related factor 2 (Nrf2) which governs antioxidant synthesis and enzymes involved in the elimination of ROS [96].
When the gut homeostasis is compromised, anti-inflammatory molecules such as SCFAs are decreased and an imbalance occurs with levels of pro-inflammatory molecules (e.g., LPS or biofilm amyloid fibres) [97,98] resulting in greater permeability of the intestinal wall, increased mitochondrial ROS production, neuronal peroxisome proliferation, as well as neurotoxin aggregation and, potentially, neurodegeneration. The decline in free radicals in the brain, through the reduction of oxidation by the modulation of the gut microbiome with the consumption of (poly)phenolic compounds, is reflected by the decrease in the level of malondialdehyde (MDA) and ROS, which is concordant with the changes in SCFAs production or the increase in SCFA-producing bacteria in several studies [74,80,82,85,99,100,101,102,103,104,105,106] (Table 1). This interplay between gut microbiota and brain oxidative stress highlights the potential of the gut microbiome to modulate the brain redox status. Furthermore, there is also a consensus regarding (poly)phenol consumption, the gut microbiome ecosystem and brain integrity, via the maintenance of BBB, improvement of synaptic activity, and the overall reduction of inflammation in the brain [68,77,80,107,108]. In some cases, there is a parallel between the observed increase in SCFA levels, or the increase in SCFA-producing bacteria and a positive regulation of astrocyte and microglial activity in the brain, hence collectively supporting neuronal activity [68,107,108].
The release of specific hormones (corticotropin, adrenocorticotropin, corticosterone or glucocorticoids and other hormones) highlights the neuroendocrine activity of (poly)phenolic compounds in addition to their neuroprotective effects. Indeed, it seems that the neuroendocrine effects of (poly)phenols could be responsible for at least part of their neuroprotective effects, as it was reported with regard to the free radical scavenging effects of oestrogen (as well as genomic effects) and the consequent neuroprotection. This is notably illustrated by an a posteriori increase in neuroinflammation, which was observed following menopause and the associated fall in oestrogen levels [109,110]. In models of (neuro)inflammatory diseases, e.g., direct administration of amyloid beta Aβ1–42 peptide [111], D-galactose [68,80,81,82,99,104,105] or by other neurotoxins [111], oxidative stress, inflammation and mitochondrial dysfunction occur, usually in parallel to an abnormal gut ecosystem. This is of major importance as it validates the bidirectionality of the gut–brain axis, with induced neuro-disorders causing deleterious changes at the level of the microbiome. A consensus between the related homeostatic dynamics of the gut microbiome with (poly)phenols and the decreased in inflammasome and overall brain inflammation (reduced cytokines levels and macrophage activities) along with overall oxidative status is also evident. This is a determining factor as it validates the mediating effects of the gut microbiome structure towards brain health and antioxidative properties, while confirming the prebiotic effects of (poly)phenolic compounds (Table 1).
Table 1.
The effects of (poly)phenols on gut microbiome structure, microbial metabolites, and related brain functions in models of neurological diseases and ageing: Results from preclinical studies.
3.2. Clinical Evidence
With regard to the clinical evidence, there is a marked lack of data, with only three human clinical studies considering the mediating effects of (poly)phenols on the gut–brain axis to date, and a notable absence of molecular mechanisms (Table 2). In addition, the current available studies reflect an emphasis on (poly)phenol-rich foods rather than isolated compounds. As far as studies recognising the effects of (poly)phenols on microbiome structure, metabolites and related functions, it is challenging to draw conclusions due to the paucity of available studies as well as the heterogeneity in design and trial duration. The clinical study conducted by Romo-Vaquero [136] in Parkinson’s disease patients shows a correlation between a decrease in gut diversity favouring a pro-inflammatory bacterial composition and a decreased production of anti-inflammatory metabolites (urolithin) as well as the SCFA butyrate. This translates into increased production of p-cresol and lipopolysaccharides (LPS), as well as increased degradation of intestinal mucus, suggesting enhanced permeability of the gut cell wall. Of interest here, the uraemic toxin p-cresol sulfate (pCS) is known to increase endothelial permeability and has been recently linked to cerebrovascular damage due to its disruptive actions on BBB integrity [61,137]. Other studies, although lacking the molecular mechanisms linked to the GBA and related derived metabolites, have evaluated the effects of olive oil polyphenols, major components of the Mediterranean diet (Med Diet). Casamenti and Stefani highlighted the prebiotic effects of (poly)phenols present in extra virgin olive oil (EVOO) in a subset of the PREDIMED trial, and their cognitive benefits [138,139]. Of interest, the Med Diet is known to preserve cognitive functions and reduce the risks of neurological diseases with effects ranging from preserved brain volumes and cognitive abilities [140], reduced cognitive decline [141] and overall inflammation during ageing [142]. However, further research is needed to investigate the impacts of polyphenols present in EVOO on the GBA and their related metabolites.
Table 2.
The effects of polyphenols on gut microbiome structure, microbial metabolites, and related brain functions in models of neurological disease and ageing: Results from Clinical studies.
4. Conclusions
A growing body of evidence from preclinical and, to a lesser extent, clinical studies, confirm the effects of various dietary (poly)phenols on brain health and ageing, acting through modulation of the GBA. However, several key points pose challenges in understanding the role of (poly)phenols and GBA. For instance, although (poly)phenols have independently demonstrated their potential in gut health and in neuronal protection, studies reporting the direct modulation of gut–brain axis and the molecular mechanisms underlying these effects are very limited. While promising, clinical studies are currently scarce, therefore limiting information regarding the translational potential of these dietary products. The need for studies and human trials that are targeted, homogeneous and with reproducible results is therefore important [60]. In this respect, future studies should focus on the mechanisms to capture the complex interaction of these food bioactives with the gut microbiota and with host systems. In addition, because ageing of the gut is generally accompanied by a decrease in microbial diversity, which is a key factor in maintaining overall gut health and functionality, forthcoming studies should investigate the older segment of the population. Emphasis should be placed on characterising the brain’s health and its related systemic biomarkers, as well as on neuroimaging, coupled with analysis of the gut microbiome, to better understand the protective role of these natural compounds on healthy brain ageing.
Author Contributions
Writing—original draft preparation, L.L. and D.V.; writing—review and editing, M.G.P., M.M., S.M., A.S.L., L.P. and D.G.; supervision, D.V. All authors have read and agreed to the published version of the manuscript.
Funding
This research received no external funding.
Conflicts of Interest
Authors Line Pourtau and David Gaudout were employed by the company Activ’Inside. The remaining authors declare that the research was conducted in the absence of any commercial or financial relationships that could be construed as a potential conflict of interest.
References
- Murman, D.L. The Impact of Age on Cognition. Semin Hear. 2015, 36, 111–121. [Google Scholar] [CrossRef] [Scilit]
- GBD 2019 Dementia Forecasting Collaborators. Estimation of the global prevalence of dementia in 2019 and forecasted prevalence in 2050: An analysis for the Global Burden of Disease Study 2019. Lancet Public Health 2022, 7, e105–e125. [Google Scholar] [CrossRef] [PubMed]
- Livingston, G.; Huntley, J.; Sommerlad, A.; Ames, D.; Ballard, C.; Banerjee, S.; Brayne, C.; Burns, A.; Cohen-Mansfield, J.; Cooper, C.; et al. Dementia prevention, intervention, and care: 2020 report of the Lancet Commission. Lancet 2020, 396, 413–446. [Google Scholar] [CrossRef] [Scilit]
- Cryan, J.F.; O’Riordan, K.J.; Cowan, C.S.M.; Sandhu, K.V.; Bastiaanssen, T.F.S.; Boehme, M.; Codagnone, M.G.; Cussotto, S.; Fulling, C.; Golubeva, A.V.; et al. The Microbiota-Gut-Brain Axis. Physiol. Rev. 2019, 99, 1877–2013. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ortega, M.A.; Álvarez-Mon, M.A.; García-Montero, C.; Fraile-Martínez, O.S.; Monserrat, J.; Martinez-Rozas, L.; Rodríguez-Jiménez, R.; Álvarez-Mon, M.; Lahera, G. Microbiota–gut–brain axis mechanisms in the complex network of bipolar disorders: Potential clinical implications and translational opportunities. Mol. Psychiatry 2023, 28, 2645–2673. [Google Scholar] [CrossRef] [Scilit]
- Rhee, S.H.; Pothoulakis, C.; Mayer, E.A. Principles and clinical implications of the brain–gut–enteric microbiota axis. Nat. Rev. Gastroenterol. Hepatol. 2009, 6, 306–314. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Rutsch, A.; Kantsjö, J.B.; Ronchi, F. The Gut-Brain Axis: How Microbiota and Host Inflammasome Influence Brain Physiology and Pathology. Front. Immunol. 2020, 11, 604179. [Google Scholar] [CrossRef] [Scilit]
- Sun, L.-J.; Li, J.-N.; Nie, Y.-Z. Gut hormones in microbiota-gut-brain cross-talk. Chin. Med. J. 2020, 133, 826–833. [Google Scholar] [CrossRef] [Scilit]
- Carabotti, M.; Scirocco, A.; Maselli, M.A.; Severi, C. The gut-brain axis: Interactions between enteric microbiota, central and enteric nervous systems. Ann. Gastroenterol. 2015, 28, 203–209. [Google Scholar]
- Ma, Q.; Xing, C.; Long, W.; Wang, H.Y.; Liu, Q.; Wang, R.-F. Impact of microbiota on central nervous system and neurological diseases: The gut-brain axis. J. Neuroinflamm. 2019, 16, 53. [Google Scholar] [CrossRef] [Scilit]
- Zheng, D.; Liwinski, T.; Elinav, E. Interaction between microbiota and immunity in health and disease. Cell Res. 2020, 30, 492–506. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ahlman, H.; Nilsson, O. The gut as the largest endocrine organ in the body. Ann. Oncol. 2001, 12, S63–S68. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, J.; Tan, Y.; Cheng, H.; Zhang, D.; Feng, W.; Peng, C. Functions of Gut Microbiota Metabolites, Current Status and Future Perspectives. Aging Dis. 2022, 13, 1106–1126. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Rowland, I.; Gibson, G.; Heinken, A.; Scott, K.; Swann, J.; Thiele, I.; Tuohy, K. Gut microbiota functions: Metabolism of nutrients and other food components. Eur. J. Nutr. 2017, 57, 1–24. [Google Scholar] [CrossRef] [Scilit]
- Daniel, H. Diet and Gut Microbiome and the “Chicken or Egg” Problem. Front. Nutr. 2022, 8, 828630. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Damiano, S.; Sozio, C.; La Rosa, G.; Guida, B.; Faraonio, R.; Santillo, M.; Mondola, P. Metabolism Regulation and Redox State: Insight into the Role of Superoxide Dismutase 1. Int. J. Mol. Sci. 2020, 21, 6606. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Narduzzi, L.; Agulló, V.; Favari, C.; Tosi, N.; Mignogna, C.; Crozier, A.; Del Rio, D.; Mena, P. (Poly)phenolic compounds and gut microbiome: New opportunities for personalized nutrition. Microbiome Res. Rep. 2022, 1, 16. [Google Scholar] [CrossRef] [Scilit]
- Tomasova, L.; Grman, M.; Ondrias, K.; Ufnal, M. The impact of gut microbiota metabolites on cellular bioenergetics and cardiometabolic health. Nutr. Metab. 2021, 18, 72. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lippolis, T.; Cofano, M.; Caponio, G.R.; De Nunzio, V.; Notarnicola, M. Bioaccessibility and Bioavailability of Diet Polyphenols and Their Modulation of Gut Microbiota. Int. J. Mol. Sci. 2023, 24, 3813. [Google Scholar] [CrossRef] [Scilit]
- Del Rio, D.; Rodriguez-Mateos, A.; Spencer, J.P.E.; Tognolini, M.; Borges, G.; Crozier, A. Dietary (Poly)phenolics in Human Health: Structures, Bioavailability, and Evidence of Protective Effects Against Chronic Diseases. Antioxid. Redox Signal. 2013, 18, 1818–1892. [Google Scholar] [CrossRef] [Scilit]
- Rodriguez-Mateos, A.; Vauzour, D.; Krueger, C.G.; Shanmuganayagam, D.; Reed, J.; Calani, L.; Mena, P.; Del Rio, D.; Crozier, A. Bioavailability, bioactivity and impact on health of dietary flavonoids and related compounds: An update. Arch. Toxicol. 2014, 88, 1803–1853. [Google Scholar] [CrossRef] [Scilit]
- Ahmed, H.; Leyrolle, Q.; Koistinen, V.; Kärkkäinen, O.; Layé, S.; Delzenne, N.; Hanhineva, K. Microbiota-derived metabolites as drivers of gut–brain communication. Gut Microbes 2022, 14, 2102878. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- de Vos, W.M.; Tilg, H.; Van Hul, M.; Cani, P.D. Gut microbiome and health: Mechanistic insights. Gut 2022, 71, 1020–1032. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Walker, A.W.; Hoyles, L. Human microbiome myths and misconceptions. Nat. Microbiol. 2023, 8, 1392–1396. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wan, X.; Yang, Q.; Wang, X.; Bai, Y.; Liu, Z. Isolation and Cultivation of Human Gut Microorganisms: A Review. Microorganisms 2023, 11, 1080. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jandhyala, S.M. Role of the normal gut microbiota. World J. Gastroenterol. 2015, 21, 8787. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Coelho, G.D.P.; Ayres, L.F.A.; Barreto, D.S.; Henriques, B.D.; Prado, M.R.M.C.; Passos, C.M.D. Acquisition of microbiota according to the type of birth: An integrative review. Rev. Lat.-Am. Enferm. 2021, 29, e3446. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, C.; Du, M.-X.; Abuduaini, R.; Yu, H.-Y.; Li, D.-H.; Wang, Y.-J.; Zhou, N.; Jiang, M.-Z.; Niu, P.-X.; Han, S.-S.; et al. Enlightening the taxonomy darkness of human gut microbiomes with a cultured biobank. Microbiome 2021, 9, 119. [Google Scholar] [CrossRef] [Scilit]
- Rothschild, D.; Weissbrod, O.; Barkan, E.; Kurilshikov, A.; Korem, T.; Zeevi, D.; Costea, P.I.; Godneva, A.; Kalka, I.N.; Bar, N.; et al. Environment dominates over host genetics in shaping human gut microbiota. Nature 2018, 555, 210–215. [Google Scholar] [CrossRef] [Scilit]
- Lawley, T.D.; Walker, A.W. Intestinal colonization resistance. Immunology 2012, 138, 1–11. [Google Scholar] [CrossRef] [Scilit]
- Rolhion, N.; Chassaing, B. When pathogenic bacteria meet the intestinal microbiota. Philos. Trans. R. Soc. B Biol. Sci. 2016, 371, 20150504. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hampel, H.; Hardy, J.; Blennow, K.; Chen, C.; Perry, G.; Kim, S.H.; Villemagne, V.L.; Aisen, P.; Vendruscolo, M.; Iwatsubo, T.; et al. The Amyloid-β Pathway in Alzheimer’s Disease. Mol. Psychiatry 2021, 26, 5481–5503. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cattaneo, A.; Cattane, N.; Galluzzi, S.; Provasi, S.; Lopizzo, N.; Festari, C.; Ferrari, C.; Guerra, U.P.; Paghera, B.; Muscio, C.; et al. Association of brain amyloidosis with pro-inflammatory gut bacterial taxa and peripheral inflammation markers in cognitively impaired elderly. Neurobiol. Aging 2017, 49, 60–68. [Google Scholar] [CrossRef] [Scilit]
- Broderick, N.A.; Buchon, N.; Lemaitre, B.; McFall-Ngai, M.J. Microbiota-Induced Changes in Drosophila melanogaster Host Gene Expression and Gut Morphology. mBio 2014, 5, 10–1128. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Walston, J.; Hadley, E.C.; Ferrucci, L.; Guralnik, J.M.; Newman, A.B.; Studenski, S.A.; Ershler, W.B.; Harris, T.; Fried, L.P. Research agenda for frailty in older adults: Toward a better understanding of physiology and etiology: Summary from the American Geriatrics Society/National Institute on Aging Research Conference on Frailty in Older Adults. J. Am. Geriatr. Soc. 2006, 54, 991–1001. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fiske, A.; Wetherell, J.L.; Gatz, M. Depression in Older Adults. Annu. Rev. Clin. Psychol. 2009, 5, 363–389. [Google Scholar] [CrossRef] [Scilit]
- Salazar, N.; Valdés-Varela, L.; González, S.; Gueimonde, M.; de los Reyes-Gavilán, C.G. Nutrition and the gut microbiome in the elderly. Gut Microbes 2016, 8, 82–97. [Google Scholar] [CrossRef] [Scilit]
- Biagi, E.; Nylund, L.; Candela, M.; Ostan, R.; Bucci, L.; Pini, E.; Nikkïla, J.; Monti, D.; Satokari, R.; Franceschi, C.; et al. Through Ageing, and Beyond: Gut Microbiota and Inflammatory Status in Seniors and Centenarians. PLoS ONE 2010, 5, e10667. [Google Scholar] [CrossRef] [Scilit]
- Stilling, R.M.; van de Wouw, M.; Clarke, G.; Stanton, C.; Dinan, T.G.; Cryan, J.F. The neuropharmacology of butyrate: The bread and butter of the microbiota-gut-brain axis? Neurochem. Int. 2016, 99, 110–132. [Google Scholar] [CrossRef] [Scilit]
- Langille, M.G.I.; Meehan, C.J.; Koenig, J.E.; Dhanani, A.S.; Rose, R.A.; Howlett, S.E.; Beiko, R.G. Microbial shifts in the aging mouse gut. Microbiome 2014, 2, 50. [Google Scholar] [CrossRef] [Scilit]
- Franceschi, C.; Campisi, J. Chronic Inflammation (Inflammaging) and Its Potential Contribution to Age-Associated Diseases. J. Gerontol. Ser. A Biol. Sci. Med. Sci. 2014, 69, S4–S9. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jackson, M.A.; Jeffery, I.B.; Beaumont, M.; Bell, J.T.; Clark, A.G.; Ley, R.E.; O’Toole, P.W.; Spector, T.D.; Steves, C.J. Signatures of early frailty in the gut microbiota. Genome Med. 2016, 8, 8. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wilmanski, T.; Diener, C.; Rappaport, N.; Patwardhan, S.; Wiedrick, J.; Lapidus, J.; Earls, J.C.; Zimmer, A.; Glusman, G.; Robinson, M.; et al. Gut microbiome pattern reflects healthy ageing and predicts survival in humans. Nat. Metab. 2021, 3, 274–286. [Google Scholar] [CrossRef] [Scilit]
- Ghosh, T.S.; Shanahan, F.; O’Toole, P.W. Toward an improved definition of a healthy microbiome for healthy aging. Nat. Aging 2022, 2, 1054–1069. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kadry, H.; Noorani, B.; Cucullo, L. A blood–brain barrier overview on structure, function, impairment, and biomarkers of integrity. Fluids Barriers CNS 2020, 17, 69. [Google Scholar] [CrossRef] [Scilit]
- Franceschi, C.; Garagnani, P.; Parini, P.; Giuliani, C.; Santoro, A. Inflammaging: A new immune–metabolic viewpoint for age-related diseases. Nat. Rev. Endocrinol. 2018, 14, 576–590. [Google Scholar] [CrossRef] [Scilit]
- Persidsky, Y.; Ramirez, S.H.; Haorah, J.; Kanmogne, G.D. Blood–brain Barrier: Structural Components and Function Under Physiologic and Pathologic Conditions. J. Neuroimmune Pharmacol. 2006, 1, 223–236. [Google Scholar] [CrossRef] [Scilit]
- Al-Obaidi, M.M.J.; Desa, M.N.M. Mechanisms of Blood Brain Barrier Disruption by Different Types of Bacteria, and Bacterial–Host Interactions Facilitate the Bacterial Pathogen Invading the Brain. Cell. Mol. Neurobiol. 2018, 38, 1349–1368. [Google Scholar] [CrossRef] [Scilit]
- Braniste, V.; Al-Asmakh, M.; Kowal, C.; Anuar, F.; Abbaspour, A.; Tóth, M.; Korecka, A.; Bakocevic, N.; Ng, L.G.; Kundu, P.; et al. The gut microbiota influences blood-brain barrier permeability in mice. Sci. Transl. Med. 2014, 6, 263ra158. [Google Scholar] [CrossRef] [Scilit]
- Hoyles, L.; Pontifex, M.G.; Rodriguez-Ramiro, I.; Anis-Alavi, M.A.; Jelane, K.S.; Snelling, T.; Solito, E.; Fonseca, S.; Carvalho, A.L.; Carding, S.R.; et al. Regulation of blood–brain barrier integrity by microbiome-associated methylamines and cognition by trimethylamine N-oxide. Microbiome 2021, 9, 235. [Google Scholar] [CrossRef] [Scilit]
- Hoyles, L.; Snelling, T.; Umlai, U.-K.; Nicholson, J.K.; Carding, S.R.; Glen, R.C.; McArthur, S. Microbiome–host systems interactions: Protective effects of propionate upon the blood–brain barrier. Microbiome 2018, 6, 55. [Google Scholar] [CrossRef] [Scilit]
- Stachulski, A.V.; Knausenberger, T.B.A.; Shah, S.N.; Hoyles, L.; McArthur, S. A host–gut microbial amino acid co-metabolite, p-cresol glucuronide, promotes blood–brain barrier integrity in vivo. Tissue Barriers 2022, 11, 2073175. [Google Scholar] [CrossRef] [Scilit]
- Cirillo, G.; Negrete-Diaz, F.; Yucuma, D.; Virtuoso, A.; Korai, S.A.; De Luca, C.; Kaniusas, E.; Papa, M.; Panetsos, F. Vagus Nerve Stimulation: A Personalized Therapeutic Approach for Crohn’s and Other Inflammatory Bowel Diseases. Cells 2022, 11, 4103. [Google Scholar] [CrossRef] [Scilit]
- Han, Y.; Wang, B.; Gao, H.; He, C.; Hua, R.; Liang, C.; Zhang, S.; Wang, Y.; Xin, S.; Xu, J. Vagus Nerve and Underlying Impact on the Gut Microbiota-Brain Axis in Behavior and Neurodegenerative Diseases. J. Inflamm. Res. 2022, 15, 6213–6230. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pellegrini, C.; Ippolito, C.; Segnani, C.; Dolfi, A.; Errede, M.; Virgintino, D.; Fornai, M.; Antonioli, L.; Garelli, F.; Nericcio, A.; et al. Pathological remodelling of colonic wall following dopaminergic nigrostriatal neurodegeneration. Neurobiol. Dis. 2020, 139, 104821. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mayer, E.A.; Tillisch, K.; Gupta, A. Gut/brain axis and the microbiota. J. Clin. Investig. 2015, 125, 926–938. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Barone, P.; Antonini, A.; Colosimo, C.; Marconi, R.; Morgante, L.; Avarello, T.P.; Bottacchi, E.; Cannas, A.; Ceravolo, G.; Ceravolo, R.; et al. The PRIAMO study: A multicenter assessment of nonmotor symptoms and their impact on quality of life in Parkinson’s disease. Mov. Disord. 2009, 24, 1641–1649. [Google Scholar] [CrossRef] [Scilit]
- Bernal-Pacheco, O.; Limotai, N.; Go, C.L.; Fernandez, H.H. Nonmotor manifestations in Parkinson disease. Neurologist 2012, 18, 1–16. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lyons, K.E.; Pahwa, R. The impact and management of nonmotor symptoms of Parkinson’s disease. Am. J. Manag. Care 2011, 17 (Suppl. S12), S308–S314. [Google Scholar]
- Chakrabarti, A.; Geurts, L.; Hoyles, L.; Iozzo, P.; Kraneveld, A.D.; La Fata, G.; Miani, M.; Patterson, E.; Pot, B.; Shortt, C.; et al. The microbiota–gut–brain axis: Pathways to better brain health. Perspectives on what we know, what we need to investigate and how to put knowledge into practice. Cell. Mol. Life Sci. 2022, 79, 80. [Google Scholar] [CrossRef] [Scilit]
- Connell, E.; Le Gall, G.; Pontifex, M.G.; Sami, S.; Cryan, J.F.; Clarke, G.; Müller, M.; Vauzour, D. Microbial-derived metabolites as a risk factor of age-related cognitive decline and dementia. Mol. Neurodegener. 2022, 17, 43. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Godos, J.; Micek, A.; Mena, P.; Del Rio, D.; Galvano, F.; Castellano, S.; Grosso, G. Dietary (Poly)phenols and Cognitive Decline: A Systematic Review and Meta-Analysis of Observational Studies. Mol. Nutr. Food Res. 2023, 68, 2300472. [Google Scholar] [CrossRef] [Scilit]
- Rodríguez-Daza, M.C.; Pulido-Mateos, E.C.; Lupien-Meilleur, J.; Guyonnet, D.; Desjardins, Y.; Roy, D. Polyphenol-Mediated Gut Microbiota Modulation: Toward Prebiotics and Further. Front. Nutr. 2021, 8, 689456. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Vaiserman, A.; Romanenko, M.; Piven, L.; Moseiko, V.; Lushchak, O.; Kryzhanovska, N.; Guryanov, V.; Koliada, A. Differences in the gut Firmicutes to Bacteroidetes ratio across age groups in healthy Ukrainian population. BMC Microbiol. 2020, 20, 221. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Morand, C.; Tomás-Barberán, F.A. Contribution of plant food bioactives in promoting health effects of plant foods: Why look at interindividual variability? Eur. J. Nutr. 2019, 58, 13–19. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, Y.; Yu, W.; Zhang, L.; Wang, M.; Chang, W. The Interaction of Polyphenols and the Gut Microbiota in Neurodegenerative Diseases. Nutrients 2022, 14, 5373. [Google Scholar] [CrossRef] [Scilit]
- Mulder, D.; Aarts, E.; Arias Vasquez, A.; Bloemendaal, M. A systematic review exploring the association between the human gut microbiota and brain connectivity in health and disease. Mol. Psychiatry 2023, 28, 5037–5061. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Song, C.; Zhang, Y.; Cheng, L.; Shi, M.; Li, X.; Zhang, L.; Zhao, H. Tea polyphenols ameliorates memory decline in aging model rats by inhibiting brain TLR4/NF-kappaB inflammatory signaling pathway caused by intestinal flora dysbiosis. Exp. Gerontol. 2021, 153, 111476. [Google Scholar] [CrossRef] [Scilit]
- Xie, J.; Song, W.; Liang, X.; Zhang, Q.; Shi, Y.; Liu, W.; Shi, X. Protective effect of quercetin on streptozotocin-induced diabetic peripheral neuropathy rats through modulating gut microbiota and reactive oxygen species level. Biomed. Pharmacother. 2020, 127, 110147. [Google Scholar] [CrossRef] [Scilit]
- Sun, Z.Z.; Li, X.Y.; Wang, S.; Shen, L.; Ji, H.F. Bidirectional interactions between curcumin and gut microbiota in transgenic mice with Alzheimer’s disease. Appl. Microbiol. Biotechnol. 2020, 104, 3507–3515. [Google Scholar] [CrossRef] [Scilit]
- Zhang, F.; Zhou, Y.; Chen, H.; Jiang, H.; Zhou, F.; Lv, B.; Xu, M. Curcumin Alleviates DSS-Induced Anxiety-Like Behaviors via the Microbial-Brain-Gut Axis. Oxidative Med. Cell. Longev. 2022, 2022, 6244757. [Google Scholar] [CrossRef] [Scilit]
- Liu, Q.; Xie, T.; Xi, Y.; Li, L.; Mo, F.; Liu, X.; Liu, Z.; Gao, J.M.; Yuan, T. Sesamol Attenuates Amyloid Peptide Accumulation and Cognitive Deficits in APP/PS1 Mice: The Mediating Role of the Gut-Brain Axis. J. Agric. Food Chem. 2021, 69, 12717–12729. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, T.J.; Feng, Y.; Liu, T.; Wu, T.T.; Chen, Y.J.; Li, X.; Li, Q.; Wu, Y.C. Fisetin Regulates Gut Microbiota and Exerts Neuroprotective Effect on Mouse Model of Parkinson’s Disease. Front. Neurosci. 2020, 14, 549037. [Google Scholar] [CrossRef] [Scilit]
- Li, X.; Khan, I.; Xia, W.; Huang, G.; Liu, L.; Law, B.Y.K.; Yin, L.; Liao, W.; Leong, W.; Han, R.; et al. Icariin enhances youth-like features by attenuating the declined gut microbiota in the aged mice. Pharmacol. Res. 2021, 168, 105587. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gao, L.; Li, J.; Zhou, Y.; Huang, X.; Qin, X.; Du, G. Effects of Baicalein on Cortical Proinflammatory Cytokines and the Intestinal Microbiome in Senescence Accelerated Mouse Prone 8. ACS Chem. Neurosci. 2018, 9, 1714–1724. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, J.; Zhang, T.; Wang, Y.; Si, C.; Wang, X.; Wang, R.T.; Lv, Z. Baicalin ameliorates neuropathology in repeated cerebral ischemia-reperfusion injury model mice by remodeling the gut microbiota. Aging 2020, 12, 3791–3806. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xia, Y.; Peng, S.; Lin, M.; Duan, H.; Yuan, F.; Shao, M.; Tan, W.; Luo, H. Apigenin attenuates visceral hypersensitivity in water avoidance stress rats by modulating the microbiota-gut-brain axis and inhibiting mast cell activation. Biomed. Pharmacother. 2023, 167, 115562. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Marques, C.; Fernandes, I.; Meireles, M.; Faria, A.; Spencer, J.P.E.; Mateus, N.; Calhau, C. Gut microbiota modulation accounts for the neuroprotective properties of anthocyanins. Sci. Rep. 2018, 8, 11341. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Si, X.; Bi, J.; Chen, Q.; Cui, H.; Bao, Y.; Tian, J.; Shu, C.; Wang, Y.; Tan, H.; Zhang, W.; et al. Effect of Blueberry Anthocyanin-Rich Extracts on Peripheral and Hippocampal Antioxidant Defensiveness: The Analysis of the Serum Fatty Acid Species and Gut Microbiota Profile. J. Agric. Food Chem. 2021, 69, 3658–3666. [Google Scholar] [CrossRef] [Scilit]
- Zhang, J.; Hao, J.; Liu, R.; Wu, T.; Liu, R.; Sui, W.; Zhang, M. Hawthorn flavonoid ameliorates cognitive deficit in mice with Alzheimer’s disease by increasing the levels of Bifidobacteriales in gut microbiota and docosapentaenoic acid in serum metabolites. Food Funct. 2022, 13, 12371–12382. [Google Scholar] [CrossRef] [Scilit]
- Gao, X.; Liu, J.; Luo, Y.; Lei, Y.; Long, W.; Wang, K.; Zhou, J.; Lei, M.; Yang, N.; Zou, H.; et al. Various Fractions of Alcoholic Extracts from Dendrobium nobile Functionalized Antioxidation and Antiaging in D-Galactose-Induced Aging Mice. Front. Biosci. (Landmark Ed.) 2022, 27, 315. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, S.; He, Y.; Zhong, S.; Li, Y.; Di, Y.; Wang, Q.; Ren, D.; Liu, S.; Li, D.; Cao, F. Antioxidant and Anti-Aging Properties of Polyphenol-Polysaccharide Complex Extract from Hizikia fusiforme. Foods 2023, 12, 3725. [Google Scholar] [CrossRef] [Scilit]
- Balasubramanian, R.; Bazaz, M.R.; Pasam, T.; Sharief, N.; Velip, L.; Samanthula, G.; Dandekar, M.P. Involvement of Microbiome Gut-Brain Axis in Neuroprotective Effect of Quercetin in Mouse Model of Repeated Mild Traumatic Brain Injury. Neuromol. Med. 2023, 25, 242–254. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, Y.; Pan, J.; Liu, Y.; Zhang, X.; Cheng, K. Effects of Ficus pandurata Hance var. angustifolia Cheng Flavonoids on Intestinal Barrier and Cognitive Function by Regulating Intestinal Microbiota. Foods 2023, 12, 1682. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sanchez-Tapia, M.; Aguilar-Lopez, M.; Perez-Cruz, C.; Pichardo-Ontiveros, E.; Wang, M.; Donovan, S.M.; Tovar, A.R.; Torres, N. Nopal (Opuntia ficus indica) protects from metabolic endotoxemia by modifying gut microbiota in obese rats fed high fat/sucrose diet. Sci. Rep. 2017, 7, 4716. [Google Scholar] [CrossRef] [Scilit]
- Li, H.; Xiao, C.; Wang, F.; Guo, X.; Zhou, Z.; Jiang, Y. Blueberry-Mulberry Extract Alleviates Cognitive Impairment, Regulates Gut Metabolites, and Inhibits Inflammation in Aged Mice. Foods 2023, 12, 860. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Du, L.; Li, J.; Zhang, X.; Wang, L.; Zhang, W.; Yang, M.; Hou, C. Pomegranate peel polyphenols inhibits inflammation in LPS-induced RAW264.7 macrophages via the suppression of TLR4/NF-kappaB pathway activation. Food Nutr. Res. 2019, 63, 3. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kim, I.T.; Ryu, S.; Shin, J.S.; Choi, J.H.; Park, H.J.; Lee, K.T. Euscaphic acid isolated from roots of Rosa rugosa inhibits LPS-induced inflammatory responses via TLR4-mediated NF-kappaB inactivation in RAW 264.7 macrophages. J. Cell. Biochem. 2012, 113, 1936–1946. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Singh, A.; Yau, Y.F.; Leung, K.S.; El-Nezami, H.; Lee, J.C.-Y. Interaction of Polyphenols as Antioxidant and Anti-Inflammatory Compounds in Brain–Liver–Gut Axis. Antioxidants 2020, 9, 669. [Google Scholar] [CrossRef] [Scilit]
- Wong, X.; Madrid, A.M.; Tralma, K.; Castillo, R.; Carrasco-Pozo, C.; Navarrete, P.; Beltrán, C.; Pastene, E.; Gotteland, M. Polyphenol extracts interfere with bacterial lipopolysaccharide in vitro and decrease postprandial endotoxemia in human volunteers. J. Funct. Foods 2016, 26, 406–417. [Google Scholar] [CrossRef] [Scilit]
- Lundin, J.I.; Checkoway, H. Endotoxin and cancer. Environ. Health Perspect. 2009, 117, 1344–1350. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Brooks, D.; Barr, L.C.; Wiscombe, S.; McAuley, D.F.; Simpson, A.J.; Rostron, A.J. Human lipopolysaccharide models provide mechanistic and therapeutic insights into systemic and pulmonary inflammation. Eur. Respir. J. 2020, 56, 1901298. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Beckhauser, T.F.; Francis-Oliveira, J.; De Pasquale, R. Reactive Oxygen Species: Physiological and Physiopathological Effects on Synaptic Plasticity. J. Exp. Neurosci. 2016, 10, 23–48. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zorov, D.B.; Plotnikov, E.Y.; Silachev, D.N.; Zorova, L.D.; Pevzner, I.B.; Zorov, S.D.; Babenko, V.A.; Jankauskas, S.S.; Popkov, V.A.; Savina, P.S. Microbiota and mitobiota. Putting an equal sign between mitochondria and bacteria. Biochemistry 2014, 79, 1017–1031. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- González-Bosch, C.; Boorman, E.; Zunszain, P.A.; Mann, G.E. Short-chain fatty acids as modulators of redox signaling in health and disease. Redox Biology 2021, 47, 102165. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kasai, S.; Shimizu, S.; Tatara, Y.; Mimura, J.; Itoh, K. Regulation of Nrf2 by Mitochondrial Reactive Oxygen Species in Physiology and Pathology. Biomolecules 2020, 10, 320. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bertani, B.; Ruiz, N. Function and Biogenesis of Lipopolysaccharides. EcoSal Plus 2018, 8, 10–1128. [Google Scholar] [CrossRef] [Scilit]
- Zhou, Y.; Blanco, L.P.; Smith, D.R.; Chapman, M.R. Bacterial amyloids. Methods Mol. Biol. 2012, 849, 303–320. [Google Scholar] [CrossRef] [Scilit]
- Luo, Y.P.; Tang, X.F.; Zhang, Y.C.; Chen, S.M.; Wu, Q.; Li, W.J. Epigallocatechin-3-gallate alleviates galactose-induced aging impairment via gut-brain communication. Food Funct. 2022, 13, 11200–11209. [Google Scholar] [CrossRef] [Scilit]
- Yang, S.; Zhou, H.; Wang, G.; Zhong, X.H.; Shen, Q.L.; Zhang, X.J.; Li, R.Y.; Chen, L.H.; Zhang, Y.H.; Wan, Z. Quercetin is protective against short-term dietary advanced glycation end products intake induced cognitive dysfunction in aged ICR mice. J. Food Biochem. 2020, 44, e13164. [Google Scholar] [CrossRef] [Scilit]
- Li, S.; Liang, T.; Zhang, Y.; Huang, K.; Yang, S.; Lv, H.; Chen, Y.; Zhang, C.; Guan, X. Vitexin alleviates high-fat diet induced brain oxidative stress and inflammation via anti-oxidant, anti-inflammatory and gut microbiota modulating properties. Free Radic. Biol. Med. 2021, 171, 332–344. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, Z.; Tan, X.; Sun, X.; Wei, J.; Li, Q.X.; Wu, Z. Isoorientin Affects Markers of Alzheimer’s Disease via Effects on the Oral and Gut Microbiota in APP/PS1 Mice. J. Nutr. 2022, 152, 140–152. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cao, B.; Zeng, M.N.; Hao, F.X.; Hao, Z.Y.; Zhang, Z.K.; Liang, X.W.; Wu, Y.Y.; Zhang, Y.H.; Feng, W.S.; Zheng, X.K. P-coumaric acid ameliorates Abeta(25-35)-induced brain damage in mice by modulating gut microbiota and serum metabolites. Biomed. Pharmacother. 2023, 168, 115825. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wei, R.; Su, Z.; Mackenzie, G.G. Chlorogenic acid combined with epigallocatechin-3-gallate mitigates D-galactose-induced gut aging in mice. Food Funct. 2023, 14, 2684–2697. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yang, L.; Wang, Y.; Zheng, G.; Li, Z.; Mei, J. Resveratrol-loaded selenium/chitosan nano-flowers alleviate glucolipid metabolism disorder-associated cognitive impairment in Alzheimer’s disease. Int. J. Biol. Macromol. 2023, 239, 124316. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Avila-Nava, A.; Noriega, L.G.; Tovar, A.R.; Granados, O.; Perez-Cruz, C.; Pedraza-Chaverri, J.; Torres, N. Food combination based on a pre-hispanic Mexican diet decreases metabolic and cognitive abnormalities and gut microbiota dysbiosis caused by a sucrose-enriched high-fat diet in rats. Mol. Nutr. Food Res. 2017, 61, 1501023. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, Y.; Cheng, L.; Liu, Y.; Zhang, R.; Wu, Z.; Cheng, K.; Zhang, X. Omics Analyses of Intestinal Microbiota and Hypothalamus Clock Genes in Circadian Disturbance Model Mice Fed with Green Tea Polyphenols. J. Agric. Food Chem. 2022, 70, 1890–1901. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, Z.J.; Chen, L.H.; Xu, J.; Xu, Q.X.; Xu, W.; Yang, X.W. Corylin ameliorates chronic ulcerative colitis via regulating the gut-brain axis and promoting 5-hydroxytryptophan production in the colon. Phytomedicine 2023, 110, 154651. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Arevalo, M.A.; Azcoitia, I.; Gonzalez-Burgos, I.; Garcia-Segura, L.M. Signaling mechanisms mediating the regulation of synaptic plasticity and memory by estradiol. Horm. Behav. 2015, 74, 19–27. [Google Scholar] [CrossRef] [Scilit]
- Brann, D.W.; Dhandapani, K.; Wakade, C.; Mahesh, V.B.; Khan, M.M. Neurotrophic and neuroprotective actions of estrogen: Basic mechanisms and clinical implications. Steroids 2007, 72, 381–405. [Google Scholar] [CrossRef] [Scilit]
- Xi, Y.; Li, H.; Yu, M.; Li, X.; Li, Y.; Hui, B.; Zeng, X.; Wang, J.; Li, J. Protective effects of chlorogenic acid on trimethyltin chloride-induced neurobehavioral dysfunctions in mice relying on the gut microbiota. Food Funct. 2022, 13, 1535–1550. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xu, Y.; Xie, M.; Xue, J.; Xiang, L.; Li, Y.; Xiao, J.; Xiao, G.; Wang, H.L. EGCG ameliorates neuronal and behavioral defects by remodeling gut microbiota and TotM expression in Drosophila models of Parkinson’s disease. FASEB J. 2020, 34, 5931–5950. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kang, J.; Wang, Z.; Cremonini, E.; Le Gall, G.; Pontifex, M.G.; Muller, M.; Vauzour, D.; Oteiza, P.I. (-)-Epicatechin mitigates anxiety-related behavior in a mouse model of high fat diet-induced obesity. J. Nutr. Biochem. 2022, 110, 109158. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xu, M.; Huang, H.; Mo, X.; Zhu, Y.; Chen, X.; Li, X.; Peng, X.; Xu, Z.; Chen, L.; Rong, S.; et al. Quercetin-3-O-Glucuronide Alleviates Cognitive Deficit and Toxicity in Abeta(1-42) -Induced AD-Like Mice and SH-SY5Y Cells. Mol. Nutr. Food Res. 2021, 65, e2000660. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yuan, T.; Chu, C.; Shi, R.; Cui, T.; Zhang, X.; Zhao, Y.; Shi, X.; Hui, Y.; Pan, J.; Qian, R.; et al. ApoE-Dependent Protective Effects of Sesamol on High-Fat Diet-Induced Behavioral Disorders: Regulation of the Microbiome-Gut-Brain Axis. J. Agric. Food Chem. 2019, 67, 6190–6201. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, N.; Feng, B.N.; Hu, B.; Cheng, Y.L.; Guo, Y.H.; Qian, H. Neuroprotection of chicoric acid in a mouse model of Parkinson’s disease involves gut microbiota and TLR4 signaling pathway. Food Funct. 2022, 13, 2019–2032. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tao, J.; An, Y.; Xu, L.; Wang, Y.; Wang, C.; Li, P.; Li, M.; Yan, D.; Wang, M.; Zhong, G.; et al. The protective role of microbiota in the prevention of MPTP/P-induced Parkinson’s disease by resveratrol. Food Funct. 2023, 14, 4647–4661. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Alonso Torrens, A.; Mitchell, C.A.; Pourshahidi, L.K.; Murphy, B.O.; Allwood, W.; Rizzetto, L.; Scholz, M.; Tuohy, K.; Pereira-Caro, G.; Moreno-Rojas, J.M.; et al. Long-term supplementation with anthocyanin-rich or -poor Rubus idaeus berries does not influence microvascular architecture nor cognitive outcome in the APP/PS-1 mouse model of Alzheimer’s disease. Int. J. Food Sci. Nutr. 2023, 74, 33–50. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Frolinger, T.; Sims, S.; Smith, C.; Wang, J.; Cheng, H.; Faith, J.; Ho, L.; Hao, K.; Pasinetti, G.M. The gut microbiota composition affects dietary polyphenols-mediated cognitive resilience in mice by modulating the bioavailability of phenolic acids. Sci. Rep. 2019, 9, 3546. [Google Scholar] [CrossRef] [Scilit]
- Ho, L.; Zhao, D.; Ono, K.; Ruan, K.; Mogno, I.; Tsuji, M.; Carry, E.; Brathwaite, J.; Sims, S.; Frolinger, T.; et al. Heterogeneity in gut microbiota drive polyphenol metabolism that influences alpha-synuclein misfolding and toxicity. J. Nutr. Biochem. 2019, 64, 170–181. [Google Scholar] [CrossRef] [Scilit]
- Shimizu, C.; Wakita, Y.; Inoue, T.; Hiramitsu, M.; Okada, M.; Mitani, Y.; Segawa, S.; Tsuchiya, Y.; Nabeshima, T. Effects of lifelong intake of lemon polyphenols on aging and intestinal microbiome in the senescence-accelerated mouse prone 1 (SAMP1). Sci. Rep. 2019, 9, 3671. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, S.; Chen, Y.; Zhang, Y.; Lv, H.; Luo, L.; Wang, S.; Guan, X. Polyphenolic Extracts of Coffee Cherry Husks Alleviated Colitis-Induced Neural Inflammation via NF-kappaB Signaling Regulation and Gut Microbiota Modification. J. Agric. Food Chem. 2022, 70, 6467–6477. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gao, A.X.; Xia, T.C.; Peng, Z.T.; Wu, Q.Y.; Zhu, Y.; Dong, T.T.; Tsim, K.W. The ethanolic extract of peanut shell attenuates the depressive-like behaviors of mice through modulation of inflammation and gut microbiota. Food Res. Int. 2023, 168, 112765. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, X.; Zhao, T.; Gu, J.; Wang, Z.; Lin, J.; Wang, R.; Duan, T.; Li, Z.; Dong, R.; Wang, W.; et al. Intake of flavonoids from Astragalus membranaceus ameliorated brain impairment in diabetic mice via modulating brain-gut axis. Chin. Med. 2022, 17, 22. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xia, C.X.; Gao, A.X.; Zhu, Y.; Dong, T.T.; Tsim, K.W. Flavonoids from Seabuckthorn (Hippophae rhamnoides L.) restore CUMS-induced depressive disorder and regulate the gut microbiota in mice. Food Funct. 2023, 14, 7426–7438. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Song, C.; Yin, Y.; Qin, Y.; Li, T.; Zeng, D.; Ju, T.; Duan, F.; Zhang, Y.; Lu, W. Acanthopanax senticosus extract alleviates radiation-induced learning and memory impairment based on neurotransmitter-gut microbiota communication. CNS Neurosci. Ther. 2023, 29 (Suppl. S1), 129–145. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Donoso, F.; Egerton, S.; Bastiaanssen, T.F.S.; Fitzgerald, P.; Gite, S.; Fouhy, F.; Ross, R.P.; Stanton, C.; Dinan, T.G.; Cryan, J.F. Polyphenols selectively reverse early-life stress-induced behavioural, neurochemical and microbiota changes in the rat. Psychoneuroendocrinology 2020, 116, 104673. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Osman, A.; Hofford, R.S.; Meckel, K.R.; Dave, Y.A.; Zeldin, S.M.; Shipman, A.L.; Lucerne, K.E.; Trageser, K.J.; Oguchi, T.; Kiraly, D.D. Dietary polyphenols drive dose-dependent behavioral and molecular alterations to repeated morphine. Sci. Rep. 2023, 13, 12223. [Google Scholar] [CrossRef] [Scilit]
- Upadhyay, P.; Tyagi, A.; Agrawal, S.; Kumar, A.; Gupta, S. Bidirectional Effect of Triphala on Modulating Gut-Brain Axis to Improve Cognition in the Murine Model of Alzheimer’s Disease. Mol. Nutr. Food Res. 2023, e2300104. [Google Scholar] [CrossRef] [Scilit]
- Upadhyay, P.; Gupta, S. Dual mode of Triphala in the reversal of cognition through gut restoration in antibiotic mediated prolonged dysbiosis condition in 5XFAD mice. Exp. Neurol. 2023, 367, 114473. [Google Scholar] [CrossRef] [Scilit]
- Hu, J.; Jiao, W.; Tang, Z.; Wang, C.; Li, Q.; Wei, M.; Song, S.; Du, L.; Jin, Y. Quercetin inclusion complex gels ameliorate radiation-induced brain injury by regulating gut microbiota. Biomed. Pharmacother. 2023, 158, 114142. [Google Scholar] [CrossRef] [Scilit]
- Ephraim, E.; Brockman, J.A.; Jewell, D.E. A Diet Supplemented with Polyphenols, Prebiotics and Omega-3 Fatty Acids Modulates the Intestinal Microbiota and Improves the Profile of Metabolites Linked with Anxiety in Dogs. Biology 2022, 11, 976. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Westfall, S.; Caracci, F.; Zhao, D.; Wu, Q.L.; Frolinger, T.; Simon, J.; Pasinetti, G.M. Microbiota metabolites modulate the T helper 17 to regulatory T cell (Th17/Treg) imbalance promoting resilience to stress-induced anxiety- and depressive-like behaviors. Brain Behav. Immun. 2021, 91, 350–368. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, Z.; Zheng, G.; Wang, N.; Liang, H.; Li, C.; Wang, Y.; Cui, Y.; Yang, L. A Flower-like Brain Targeted Selenium Nanocluster Lowers the Chlorogenic Acid Dose for Ameliorating Cognitive Impairment in APP/PS1 Mice. J. Agric. Food Chem. 2023, 71, 2883–2897. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- He, H.; Qin, Q.; Xu, F.; Chen, Y.; Rao, S.; Wang, C.; Jiang, X.; Lu, X.; Xie, C. Oral polyphenol-armored nanomedicine for targeted modulation of gut microbiota-brain interactions in colitis. Sci. Adv. 2023, 9, eadf3887. [Google Scholar] [CrossRef] [Scilit]
- Romo-Vaquero, M.; Fernandez-Villalba, E.; Gil-Martinez, A.L.; Cuenca-Bermejo, L.; Espin, J.C.; Herrero, M.T.; Selma, M.V. Urolithins: Potential biomarkers of gut dysbiosis and disease stage in Parkinson’s patients. Food Funct. 2022, 13, 6306–6316. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Shah, S.N.; Knausenberger, T.B.A.; Connell, E.; Gall, G.L.; Hardy, T.A.J.; Randall, D.W.; McCafferty, K.; Yaqoob, M.M.; Solito, E.; Müller, M.; et al. Cerebrovascular damage caused by the gut microbe-derived uraemic toxin p-cresol sulfate is prevented by blockade of the epidermal growth factor receptor. bioRxiv 2022. bioRxiv:11.12.516113. [Google Scholar] [CrossRef] [Scilit]
- Bucciantini, M.; Leri, M.; Nardiello, P.; Casamenti, F.; Stefani, M. Olive Polyphenols: Antioxidant and Anti-Inflammatory Properties. Antioxidants 2021, 10, 1044. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Casamenti, F.; Stefani, M. Olive polyphenols: New promising agents to combat aging-associated neurodegeneration. Expert. Rev. Neurother. 2017, 17, 345–358. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Luciano, M.; Corley, J.; Cox, S.R.; Valdés Hernández, M.C.; Craig, L.C.A.; Dickie, D.A.; Karama, S.; McNeill, G.M.; Bastin, M.E.; Wardlaw, J.M.; et al. Mediterranean-type diet and brain structural change from 73 to 76 years in a Scottish cohort. Neurology 2017, 88, 449–455. [Google Scholar] [CrossRef] [Scilit]
- Tor-Roca, A.; Sánchez-Pla, A.; Korosi, A.; Pallàs, M.; Lucassen, P.J.; Castellano-Escuder, P.; Aigner, L.; González-Domínguez, R.; Manach, C.; Carmona, F.; et al. A Mediterranean Diet-Based Metabolomic Score and Cognitive Decline in Older Adults: A Case–Control Analysis Nested within the Three-City Cohort Study. Mol. Nutr. Food Res. 2023, 2300271. [Google Scholar] [CrossRef] [Scilit]
- Huhn, S.; Kharabian Masouleh, S.; Stumvoll, M.; Villringer, A.; Witte, A.V. Components of a Mediterranean diet and their impact on cognitive functions in aging. Front. Aging Neurosci. 2015, 7, 132. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wood, E.; Hein, S.; Mesnage, R.; Fernandes, F.; Abhayaratne, N.; Xu, Y.; Zhang, Z.; Bell, L.; Williams, C.; Rodriguez-Mateos, A. Wild blueberry (poly)phenols can improve vascular function and cognitive performance in healthy older individuals: A double-blind randomized controlled trial. Am. J. Clin. Nutr. 2023, 117, 1306–1319. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Park, M.; Choi, J.; Lee, H.J. Flavonoid-Rich Orange Juice Intake and Altered Gut Microbiome in Young Adults with Depressive Symptom: A Randomized Controlled Study. Nutrients 2020, 12, 1815. [Google Scholar] [CrossRef] [Scilit] [PubMed]
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2024 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).