


Abstract
Many viruses, such as human herpesviruses, may be present in the human oral cavity, but most are usually asymptomatic. However, if individuals become immunocompromised by age, illness, or as a side effect of therapy, these dormant viruses can be activated and produce a variety of pathological changes in the oral mucosa. Unfortunately, available treatments for viral infectious diseases are limited, because (1) there are diseases for which no treatment is available; (2) drug-resistant strains of virus may appear; (3) incomplete eradication of virus may lead to recurrence. Rational design strategies are widely used to optimize the potency and selectivity of drug candidates, but discovery of leads for new antiviral agents, especially leads with novel structures, still relies mostly on large-scale screening programs, and many hits are found among natural products, such as extracts of marine sponges, sea algae, plants, and arthropods. Here, we review representative viruses found in the human oral cavity and their effects, together with relevant antiviral compounds derived from natural products. We also highlight some recent emerging pharmaceutical technologies with potential to deliver antivirals more effectively for disease prevention and therapy.
1. Introduction
The human oral cavity is home to a rich microbial flora, including bacteria, fungi, and viruses. Oral tissues are constantly exposed to these microbes, which form a complex ecological community that influences oral and systemic health [1]. Discussion of the microbiological aspects of oral disease traditionally focuses on bacteria and fungi, but viruses are attracting increasing attention as pathogens. Viruses are generally more difficult to detect among pathogenic microbes, at least with traditional methods such as in vitro cultivation; however, the development of sophisticated molecular tools, including monoclonal antibodies and viral genome sequencing, have greatly advanced the field of virology over the past decade or so. A number of viruses have been found in the oral cavity, of which many are thought to be involved in the development of various types of oral ulcers, oral tumors, classical oral infectious diseases, and periodontitis. For example, herpes simplex virus 1 (HSV-1) causes gingivostomatitis, and the virus can subsequently enter a dormant state in the trigeminal ganglion. Blood-borne viruses such as human immunodeficiency virus (HIV) can enter the mouth via gingival crevicular fluid, and viruses causing upper respiratory tract infections are also found in the mouth [2]. Similarly, the mumps virus is known to infect the salivary glands and can be found in saliva of affected individuals. Human papillomavirus (HPV) is responsible for several oral conditions, including papilloma, condylomas, and focal epithelial hyperplasia, and has also been implicated in head and neck squamous cell carcinoma.
The field of antiviral research acquired new urgency since the 1980s, owing to the global spread of HIV, which causes acquired immune deficiency syndrome (AIDS). HIV is a member of the RNA retroviruses, which contain a reverse transcriptase (RT) enzyme that transcribes RNA into DNA in infected cells, leading to integration of the retroviral genomic information into chromosomal DNA of the host cell. Antiretroviral drugs (ARVs) often target RT, but are always given in combination with other ARVs for antiretroviral therapy (ART) in order to increase efficacy and reduce the development of resistance. The anti-HIV agent zidovudine (AZT) is a representative ARV, and was the first to be approved in the United States in 1986; however, recently, many new classes of drugs have been introduced [3], together with new formulations such as long-acting depot-type anti-HIV drugs and easy-to-use gel formulations for preventing rectal HIV infection [4].
The enormous research effort directed at the treatment of HIV has led to important advances in basic science and many therapeutic breakthroughs, including the development of inhibitors targeting a range of human viruses. Nevertheless, large-scale screening of natural products, such as extracts of marine sponges, sea algae, plants, and arthropods, remains an important source of leads for new antiviral agents, whose potency and selectivity can then be optimized with the aid of rational design strategies, including computational approaches. Thus, the aim of this review is to provide a personal viewpoint on natural-product-derived antiviral agents that are available for the treatment of pathogenic viruses, especially HIV, that may cause symptoms in the oral cavity, considered from a historic perspective. As major candidates for viruses involved in oral diseases, we focus on (1) HSV-1 and HSV-2; (2) Epstein–Barr virus (EBV); (3) Kaposi sarcoma-associated herpesvirus (KSHV); (4) human papilloma virus (HPV); and (5) HIV.
2. Viruses Associated with Oral Diseases of Humans
Members of the human herpesvirus (HHV) family cause common primary viral infections of the oral mucous membrane, and may also play a role in periodontitis. There are eight members of the HHV family, which are among the largest and most complex human viruses. We focus here on HSV-1, HSV-2, EBV, and KSHV; the others are varicella-zoster virus (VZV), human cytomegalovirus (HCMV), HHV-6, and HHV-7 (Table 1). HPV is a diverse family of viruses, which can cause a variety of pathologies, including oral squamous cell carcinoma, and chronic infection of the skin or mucosal epithelium. Furthermore, the retrovirus HIV causes a decline in immunocompetence, which can lead to various cutaneous manifestations [5]. In this section, we present a brief overview of these viruses.
Table 1.
Human herpesviruses (HHVs) and their associated diseases.
2.1. HSV-1 and HSV-2
HSVs are relatively large, enveloped, double-stranded DNA viruses with icosahedral symmetry. Infections by HSV-1 are referred to as upper body infections to distinguish them from the genital infection caused by HSV-2. The formal designations of these viruses are human herpesvirus 1 (HHV-1) and 2 (HHV-2). Oral herpes is a viral infection mainly around the mouth and lips caused by herpes simplex viruses. HSV-1 causes painful sores on the upper and lower lips, gums, tongue, roof of the mouth, inside the cheeks or nose, and sometimes on the face, chin, and neck. In addition, HSV-1 can cause symptoms such as swollen lymph nodes, fever, and muscle aches. HSV-2 is primarily associated with the genitals and most often causes genital herpes. However, it may spread to the mouth during oral sex, causing oral herpes. HSVs characteristically establish latent infection in sensory nerve ganglia, and, in this case, signs appear only when the virus is reactivated. Following recovery from primary oropharyngeal infection, the individual retains HSV DNA in the trigeminal ganglion, but the virus becomes dormant. Infected individuals have at least a 50% chance of suffering sporadic recurrent attacks of herpes labialis (otherwise known as facial herpes, herpes simplex, fever blisters, or cold sores) from time to time throughout the remainder of their life.
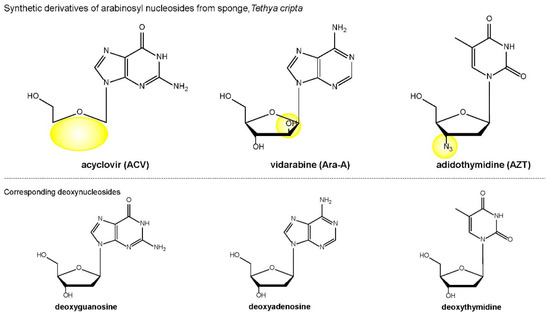
At present, the drug of choice for the treatment of HSV infections is acyclovir (ACV; 9-(2-hydroxyethoxymethyl)guanine). Its unique advantage over earlier nucleoside derivatives is that HSV-encoded thymidine kinase (TK), which has broader specificity than cellular TK, phosphorylates ACV to ACV-monophosphate (ACV-P). A cellular guanosine monophosphate (GMP) kinase then completes the phosphorylation to generate the active agent, ACV-triphosphate (ACV-PPP). ACV-PPP acts as both an inhibitor and a substrate of the viral enzyme, competing with guanosine triphosphate (GTP) for incorporation into DNA; this results in chain termination, because ACV lacks the 3’-hydroxyl group required for chain elongation. Before ACV was introduced, vidarabine (Ara-A) which was the first nucleoside analog antiviral to be systemically administered, was used. Ara-A is also sequentially phosphorylated by kinases to afford the triphosphate ara-ATP, which competitively inhibits deoxyATP (dATP). However, the mechanism of Ara-A is different in that all three phosphorylations are mediated by host adenosine kinases, resulting in a lack of specificity. Indeed, Ara-A is more toxic and less metabolically stable than ACV, although it is still employed against ACV-resistant strains. In addition, valaciclovir (VACV), an ester of ACV, is a prodrug that has greater oral bioavailability than ACV. VACV provides high plasma levels of the parent compound and offers greater efficacy, as well as decreased dosing frequency. Additionally, guanosine analog famciclovir (FCV) is another choice for the treatment of HSV infections.
2.2. EBV
EBV, formally human herpesvirus 4 (HHV-4), has a small DNA genome, and its main host cells are B lymphocytes and epithelial cells. EBV replicates in epithelial cells of the nasopharynx and salivary glands, especially the parotid, lysing them and releasing infectious virions into saliva. EBV attaches to B lymphocytes via binding of the viral glycoprotein gp350/EBV to CD21 receptors on the lymphocyte. The major characteristic of infected B lymphocytes is transformation. When this occurs, only a small amount of the viral DNA integrates into the host chromosome, and most of the viral DNA stays in a separate circular episome form. The B lymphocytes infiltrating the lymphatic tissue of the infected oropharyngeal mucosa may, in turn, become infected, but are generally not permissive for virus production. EBV is transmitted only after repeated contact with infected individuals. It can manifest in the oral cavity and/or head and neck region, e.g., as Burkitt’s lymphoma (BL), mononucleosis, or oral hairy leukoplakia (OHL), and the prevalence and disease severity are increased in individuals co-infected with HIV. Mononucleosis is common, irrespective of HIV infection status, and is associated with a primary EBV infection during adolescence and young adulthood. OHL is an oral mucosal lesion that is associated with EBV infection and is often asymptomatic, commonly presenting as non-removable white patches on the lateral borders of the tongue. OHL is now an established phenomenon in a range of conditions affecting immune competence, e.g., in immunosuppressed patients with HIV infection or bone marrow transplant recipients [6]. EBV-positive Hodgkin’s and non-Hodgkin’s lymphomas may manifest in the head and neck. Nasopharyngeal carcinoma (NPC) is also a head and neck cancer associated with EBV infection. No effective anti-EBV drugs have yet been developed. EBV is sensitive to ACV in vitro, but systemic administration of this drug has little effect on clinical illness.
2.3. KSHV
The formal designation of human herpesvirus 8 (HHV-8) was proposed for KSHV, in keeping with the systematic nomenclature adopted for all human herpesviruses. KSHV is the causative virus of Kaposi sarcoma (KS), multicentric Castleman’s disease, and primary effusion lymphoma. Humans are thought to be the natural host for KSHV, which is primarily transmitted via saliva. Infection occurs during childhood and increases with age. KSHV is detected in endothelial and spindle cells of Kaposi sarcoma lesions, as well as in circulating endothelial cells, primary effusion lymphoma cells, B lymphocytes, macrophages, dendritic cells, oropharynx and prostatic glandular epithelium, and keratinocytes. Epidemiological studies indicate that there are four clinical variants of KS: (1) classic; (2) endemic (African); (3) iatrogenic (transplant-associated); and (4) HIV/AIDS-associated (epidemic) (HIV-KS). It is well known that KS is an AIDS-defining illness and the most frequent AIDS-associated neoplasm. HIV-KS commonly affects the oral cavity, with the oral mucosa being the initial site of clinical disease in 20% of patients [7]. ART has successfully decreased the prevalence and incidence of HIV-KS. A liposome-encapsulated form of doxorubicin (Doxil) is often used primarily for the treatment of AIDS-related KS.
2.4. HPV
HPV is a small, non-enveloped, double-stranded DNA virus with icosahedral symmetry. There is wide genetic diversity among HPVs, and more than 70 genotypes of HPVs have been identified so far. Some of them are associated with a variety of benign papillomatous lesions of the skin and squamous mucosa. The mechanism of malignant transformation is not fully understood and is difficult to study because HPV is difficult to grow in culture. It is thought that the viral DNA remains episomal in benign lesions, whereas it is integrated into host chromosomal DNA in malignant cells, e.g., cervical carcinoma. Oral papillomas of the conventional kind can be caused by sexually transmitted HPV types 6, 11, and 16. Common warts are most frequently caused by type 2 [8].
HPVs induce benign tumors of the epithelium in their natural host. The discovery of the role of HPV in cervical cancer has led to the widespread use of HPV vaccines for young women, but it is still uncertain whether HPV actually plays an essential role [9]. Based on their putative role in cervical carcinoma, the viruses are classified as having either high (primarily 16 and 18) or low (primarily 6 and 11) oncogenic potential. HPVs are often found in oral samples from healthy mouths, such as brush samples of mucosa, but their prevalence is typically reported to be higher in biopsies from oral lesions, including leukoplakia and/or cancers. The association with oncogenic HPVs is less obvious in the case of leukoplakia, while there are many reports of HPVs in malignant cancers. The observed prevalence in oral cancers is considerably lower than that in cervical cancers, but the case for a role of HPVs is still reasonably strong [2]. When generations who have received papillomavirus vaccines grow up, we should find out whether the prevalence of oral carcinomas declines along with the expected decline in cervical cancer. Imiquimod is used as a patient-applied cream to treat genital warts. Imiquimod is a Toll-like receptor 7 (TLR7) agonist, promoting the secretion of inflammatory cytokines. Traditional treatments consist of locally destructive techniques, such as cautery, surgical excision, and cryotherapy using liquid nitrogen.
2.5. HIV
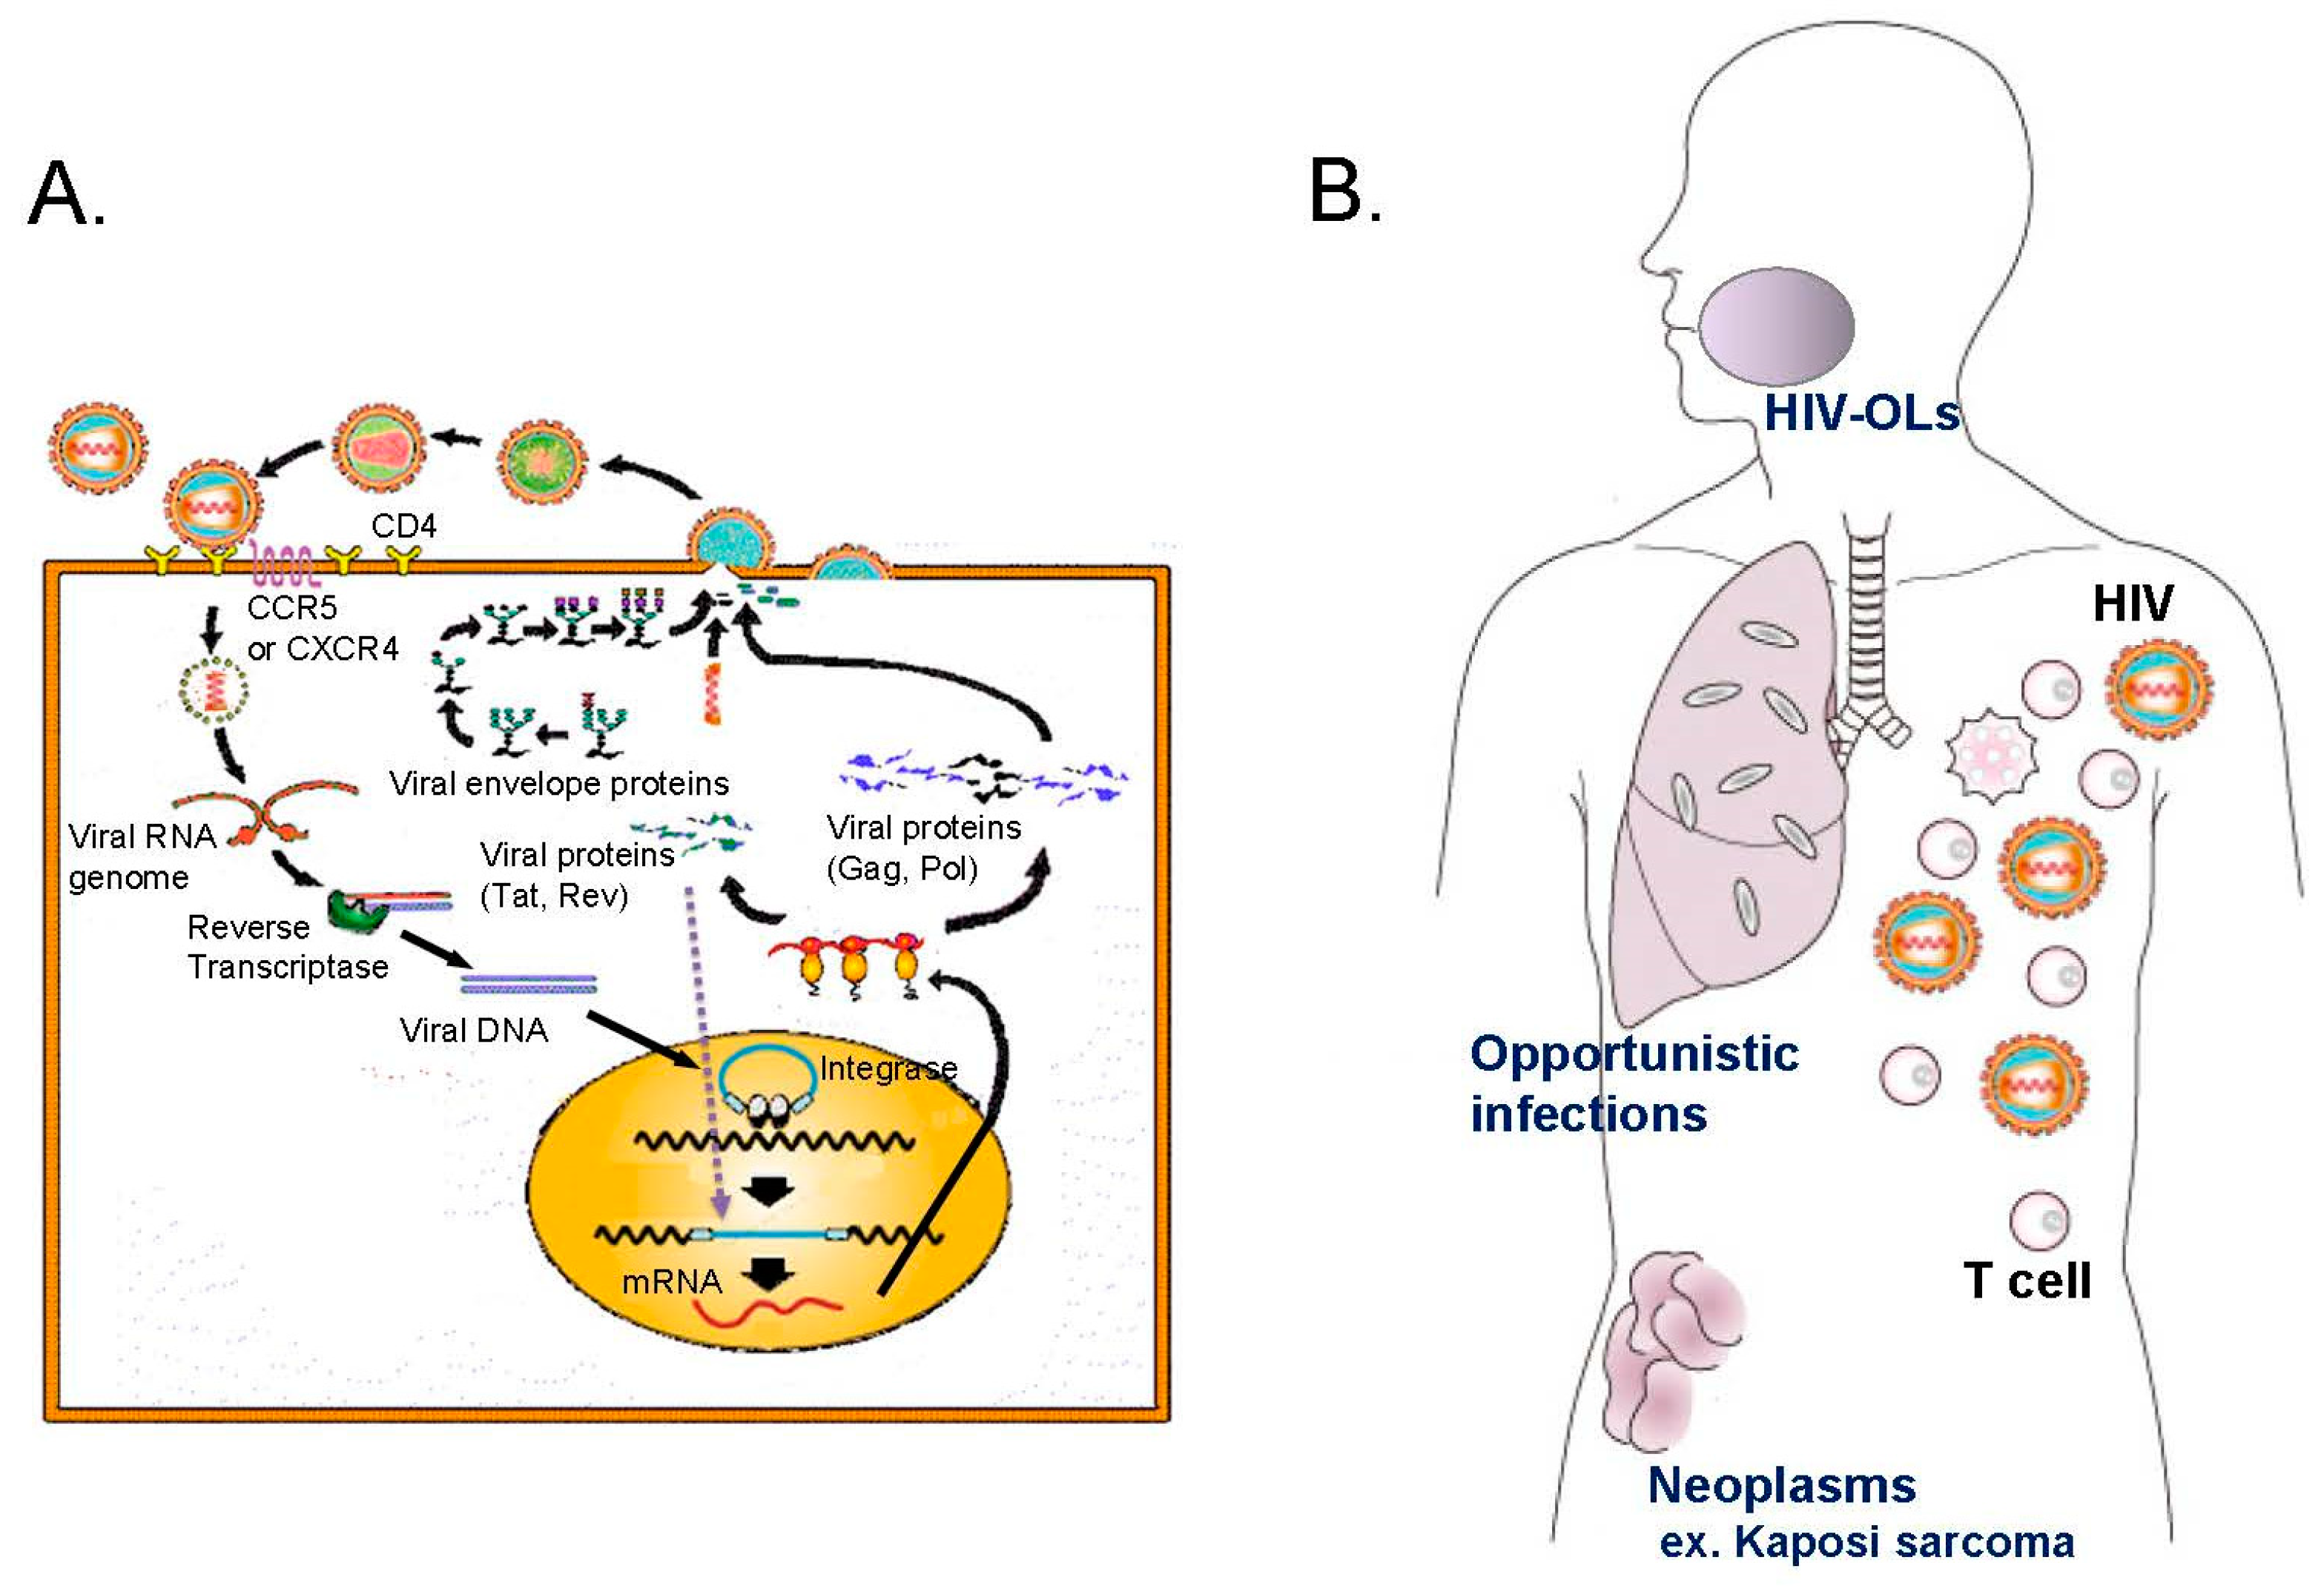
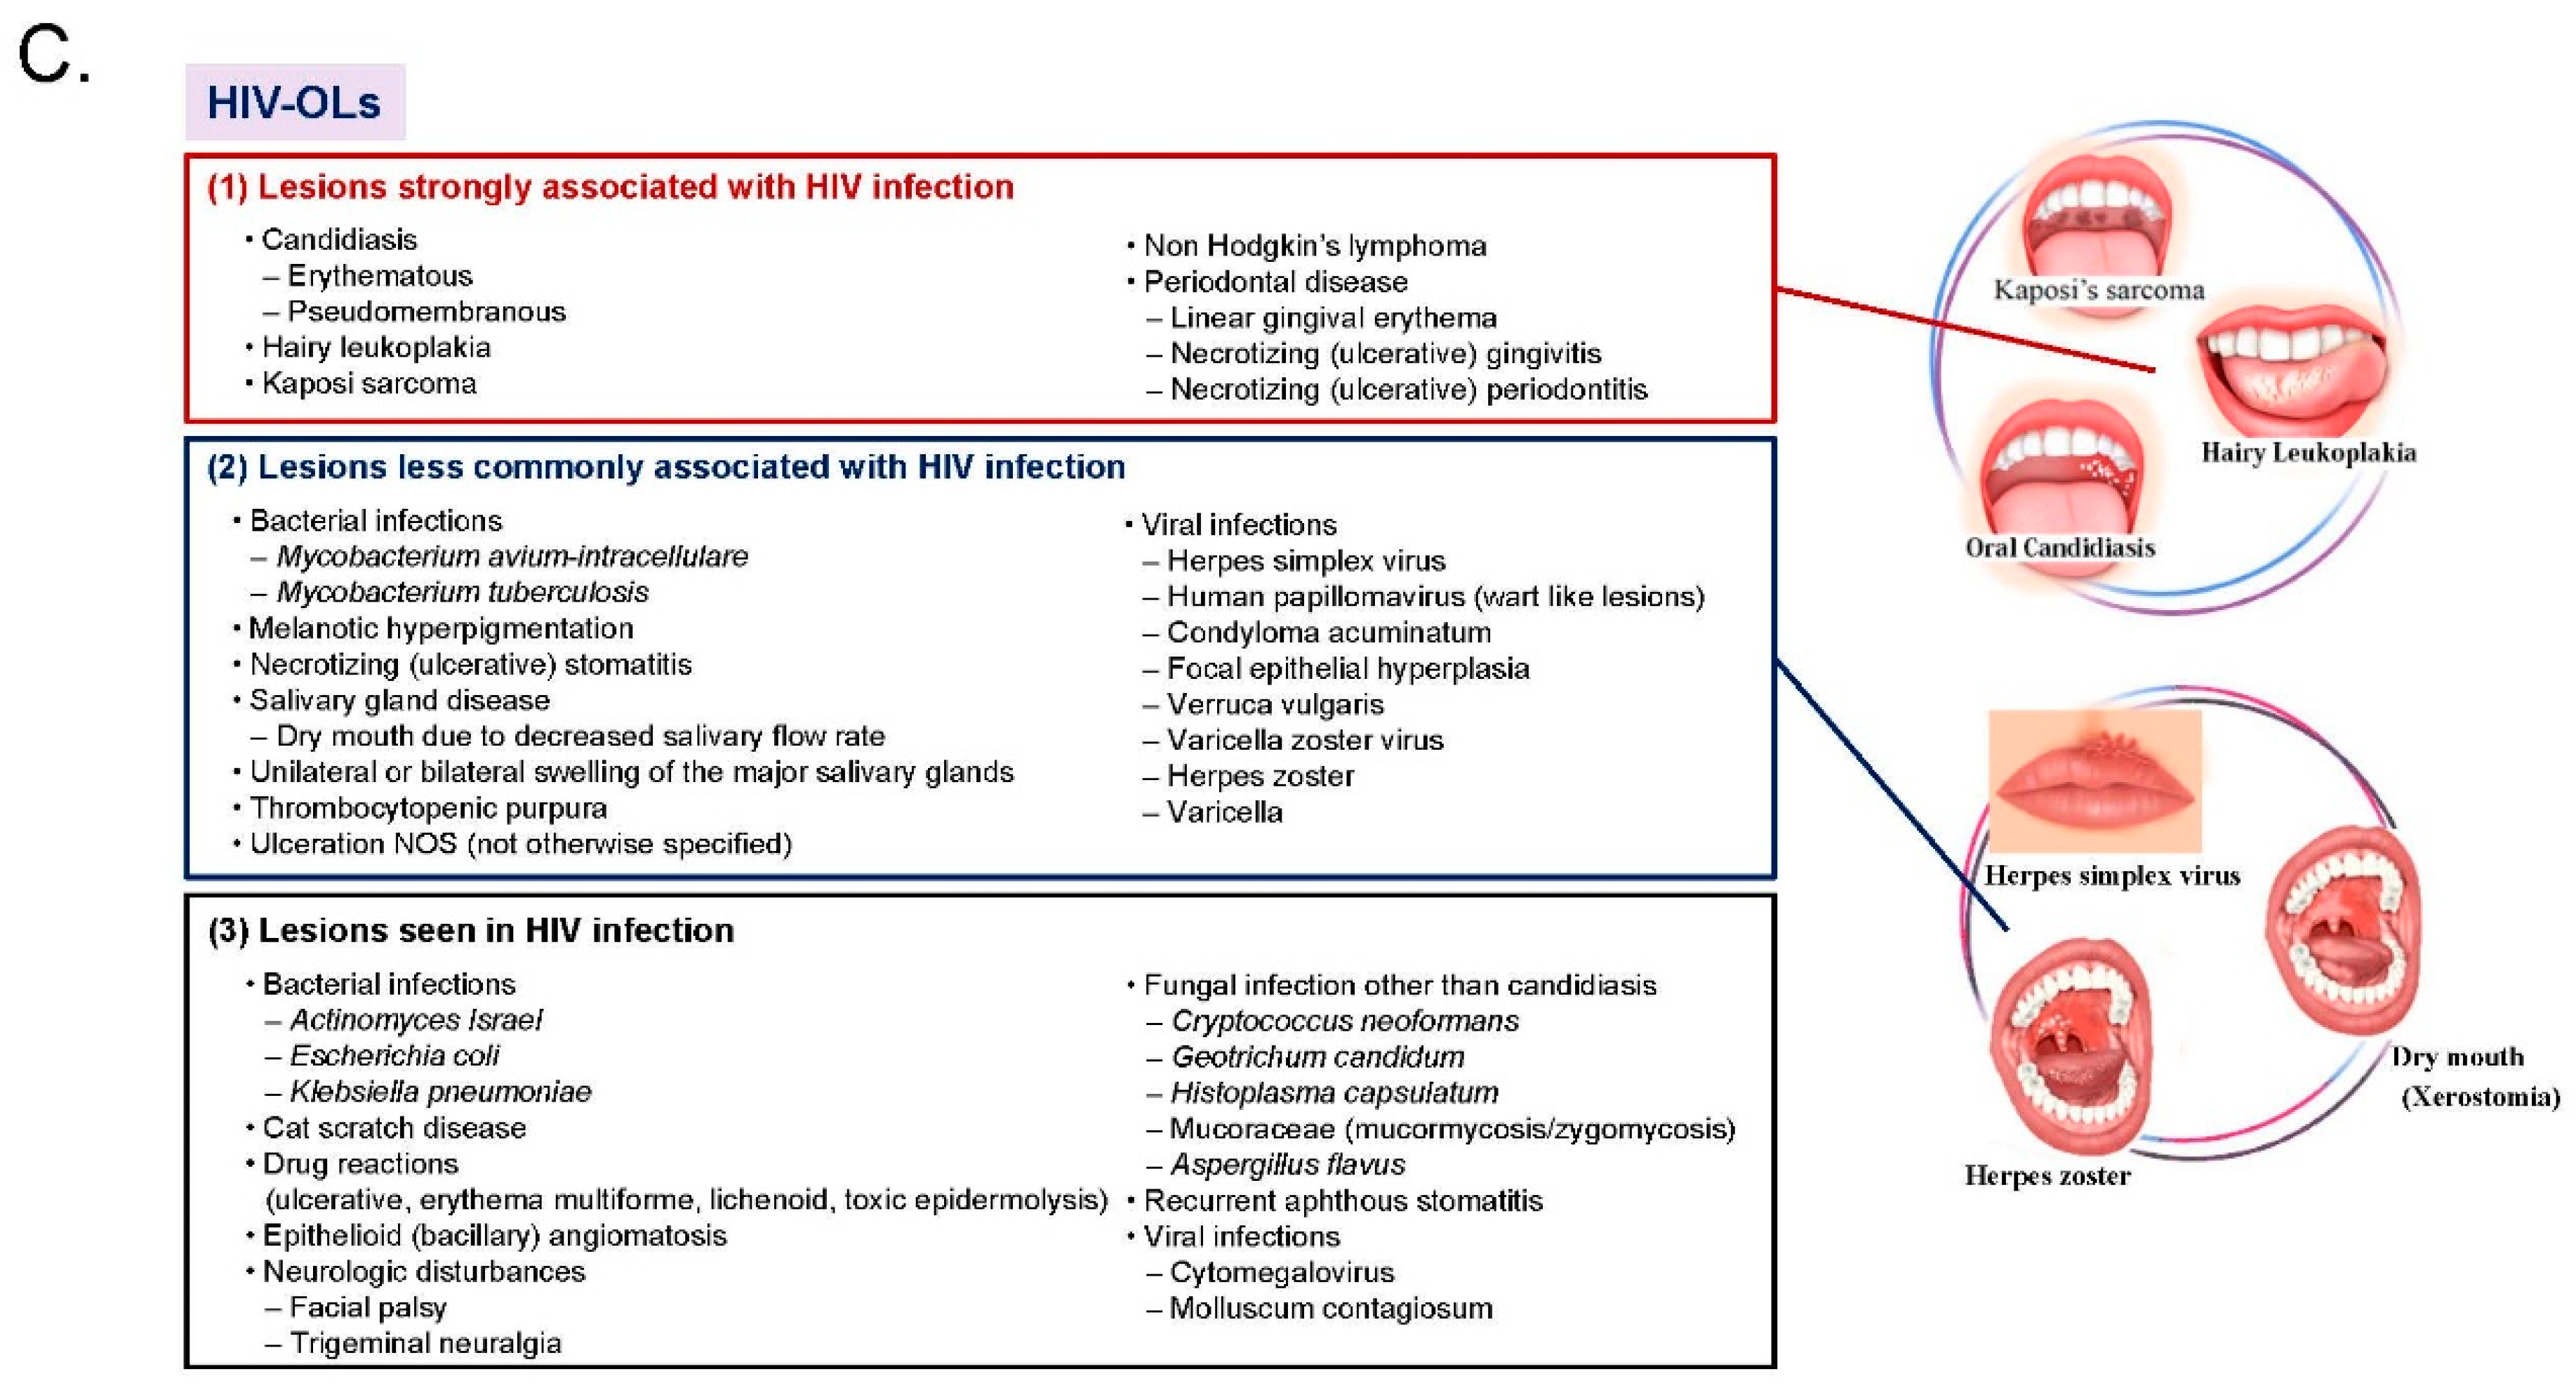
HIV is an enveloped retrovirus that is transmitted through sexual contact or by contact with infected body fluids. Retroviral RT allows the virus to integrate its genetic information into the host chromosome. HIV targets CD4-positive T-helper cells, and the resulting development of immunodeficiency leads to AIDS. Viral infections are a significant cause of morbidity and mortality in immunosuppressed patients. In general, diseases or medical treatments that have cytostatic or cytotoxic effects on lymphocytes increase the risk of viral infections, and the viral infection rate depends on the nature and degree of immunosuppression. The reactivation of latent virus is the most important determinant of the type of viral infection, and this occurs most commonly in immunosuppressed patients. Skin and mucous membrane manifestations of HIV infection may result from opportunistic disorders secondary to the decline in immunocompetence caused by the infection. HIV-related oral conditions occur in a large proportion of patients, and frequently are misdiagnosed or inadequately treated. Dental expertise is necessary for appropriate management of oral manifestations of HIV infection; however, in practice, many patients do not receive adequate dental care. Common or notable HIV-related oral conditions include the following symptoms: xerostomia (dry mouth), candidiasis, OHL, periodontal diseases such as linear gingival erythema and necrotizing ulcerative periodontitis, KS, HPV-associated warts, ulcerative conditions including HSV lesions, recurrent aphthous ulcers, and neutropenic ulcers. In 1993, consensus was reached on the classification of the oral manifestations of HIV, so-called the 1993 EC-Clearinghouse classification. It classifies oral lesions associated with HIV (HIV-OLs) into three groups: (1) lesions strongly associated with HIV infection; (2) those less commonly associated with HIV infection; and (3) lesions seen in HIV infection [10]. The sequence of events associated with HIV infection, from the cellular level of infection to oral manifestations in HIV-infected patients, is illustrated in Figure 1, together with the classification of HIV-OLs.
Figure 1.
Life cycle and effects of human immunodeficiency virus (HIV). (A) The HIV infection of cells begins when the envelope glycoprotein of a viral particle binds to both cluster of differentiation 4 (CD4) and a co-receptor that is a member of the chemokine receptor family. Once inside the cells, the viral genome is reverse-transcribed into DNA and incorporated into the cellular genome. Viral gene transcription and viral reproduction are stimulated by signals that normally activate the host cell. Production of the virus is accompanied by cell death. (B) Infection with HIV induces immunosuppression, which in turn enables many kinds of bacteria, fungi, and viruses to grow in the oral cavity. HIV-infected individuals usually exhibit immune dysfunction prior to depletion of their CD4-positive T-helper cells. The progressive immune deficiency is accompanied by a wide range of opportunistic infections and neoplasms, such as candidiasis, Kaposi sarcoma, and hairy leukoplakia, in the oral cavity. (C) The 1993 EC-Clearinghouse classification for oral lesions associated with HIV (HIV-OLs) is still globally used, despite some controversy as to its current relevance to periodontal diseases.
HIV is one of the best-studied viruses and, thus, anti-HIV agents show the widest range of structural variation among antiviral agents. Since the introduction of combination therapy (ART) for patients, HIV infection has been transformed into a long-term and manageable disorder; indeed, ART can reduce plasma virus titers to below detectable levels for more than one year and slow the disease progression. The major classes of drugs used in ART regimens include entry inhibitors (EI), nucleoside reverse-transcriptase inhibitors (NRTI), non-nucleoside reverse-transcriptase inhibitors (NNRTI), protease inhibitors (PI), and integrase strand-transfer inhibitors (INSTI).
5. Prospects
Most viral infections of the oral cavity involve HHVs, especially in HIV-infected individuals. As described in Section 2, HSV type 1 (HHV-1) and 2 (HHV-2) produce shallow, small, painful ulcers which may coalesce. The development of antiviral agents with their delivery systems that successfully stop the recurrence of oral ulceration (recurrent aphthous stomatitis (RAS)) is anticipated [96]. VZV (HHV-3) is responsible for chickenpox upon primary infection, and shingles in its reactivated form. EBV (HHV-4) causes infectious mononucleosis and/or glandular fever. HCMV (HHV-5) can cause large, painful ulceration on any oral surface. EBV and HCMV were also reported to associate with periodontitis [97]; therefore, the discovery of new antiviral agents is necessary, especially for chronic periodontitis. HHV-6 and -7 are associated with facial rashes in babies and oral ulceration. Also, reactivated HHV-6 can cause encephalitis in patients after transplantation [98]. KSHV (HHV-8) is associated with KS in AIDS patients. In HIV-infected individuals, herpes infections often persist for long period of time. In addition, HPV infections are also found in AIDS patients, and may give rise to exophytic warts, often at the corners of the mouth. In patients with AIDS, there is a danger that viremias may spread to life-threatening sites, and early treatment of oral herpetic infections is essential.
Recent developments in anti-HIV drugs has mainly been focused on creating novel formulations to improve medication compliance, such as mixed formulations including drugs with different mechanisms of action in a single tablet. For example, Complera® is a once-a-day medication, consisting of a single tablet containing rilpivirine (NNRTI), emtricitabine (NRTI), and tenofovir (NRTI). Prezcobix® utilizes a pharmacokinetic (PK) booster strategy, with a single tablet containing darunavir (PI) and a cytochrome P450 3A (CYP3A) inhibitor to prolong the blood half-life of darunavir. We have reported a depot strategy for the peptide drug Fuzeon®, which is used for the treatment of HIV-infected individuals and AIDS patients with multidrug-resistant HIV infections [99]. Natural-product-derived peptides with anti-viral activity may be candidates for PrEP and post-exposure therapy if appropriate pharmaceutical technology is employed. Also, there is still an enormous range of natural resources (plants, etc.) that remain to be explored for new antiviral candidates. Thus, discovery and development of new drugs in combination with improved pharmaceutical formulation technologies offers great promise for the future treatment of viral infections.
Author Contributions
D.A. wrote the first draft of the manuscript and reviewed it under research supervision by H.N. H.N. reviewed and edited the manuscript.
Funding
This work was supported by Grant-in-Aid for Scientific Research (C) (15K01319 and 17K08254) of Japan.
Acknowledgments
We thank the members of the Department of Microbiology, St. Marianna University School of Medicine, and the Department of Microbiology and Immunology, Kagoshima University Dental School, for much helpful discussion and technical support. We also thank Dr. Nobutaka Fujii (Kyoto University), Dr. Hiroshi Sakagami (Meikai University), and Dr. Naoki Yamamoto (Tokyo Medical and Dental University) for collaboration in our research on anti-HIV compounds.
Conflicts of Interest
The authors declare no conflicts of interest.
References
- Aas, J.A.; Paster, B.J.; Stokes, L.N.; Olsen, I.; Dewhirst, F.E. Defining the normal bacterial flora of the oral cavity. J. Clin. Microbiol. 2005, 43, 5721–5732. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Grinde, B.; Olsen, I. The role of viruses in oral disease. J. Oral Microbiol. 2010, 2. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Caplan, M.R.; Daar, E.S.; Corado, K.C. Next generation fixed dose combination pharmacotherapies for treating HIV. Expert Opin. Pharmacother. 2018, 19, 589–596. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dobard, C.W.; Taylor, A.; Sharma, S.; Anderson, P.L.; Bushman, L.R.; Chuong, D.; Pau, C.P.; Hanson, D.; Wang, L.; Garcia-Lerma, J.G.; et al. Protection Against Rectal Chimeric Simian/Human Immunodeficiency Virus Transmission in Macaques by Rectal-Specific Gel Formulations of Maraviroc and Tenofovir. J. Infect. Dis. 2015, 212, 1988–1995. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cedeno-Laurent, F.; Gomez-Flores, M.; Mendez, N.; Ancer-Rodriguez, J.; Bryant, J.L.; Gaspari, A.A.; Trujillo, J.R. New insights into HIV-1-primary skin disorders. J. Int. AIDS Soc. 2011, 14, 5. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Khammissa, R.A.; Fourie, J.; Chandran, R.; Lemmer, J.; Feller, L. Epstein-Barr Virus and Its Association with Oral Hairy Leukoplakia: A Short Review. Int. J. Dent. 2016, 2016, 4941783. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Khammissa, R.A.; Pantanowitz, L.; Feller, L. Oral HIV-Associated Kaposi Sarcoma: A Clinical Study from the Ga-Rankuwa Area, South Africa. AIDS Res. Treat. 2012, 2012, 873171. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cubie, H.A. Diseases associated with human papillomavirus infection. Virology 2013, 445, 21–34. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Giuliano, A.R.; Tortolero-Luna, G.; Ferrer, E.; Burchell, A.N.; de Sanjose, S.; Kjaer, S.K.; Munoz, N.; Schiffman, M.; Bosch, F.X. Epidemiology of human papillomavirus infection in men, cancers other than cervical and benign conditions. Vaccine 2008, 26 (Suppl. 10), K17–K28. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Classification and Diagnostic Criteria for Oral Lesions in HIV Infection. EC-Clearinghouse on Oral Problems Related to HIV Infection and WHO Collaborating Centre on Oral Manifestations of the Immunodeficiency Virus. J. Oral Pathol. Med. 1993, 22, 289–291. [Google Scholar] [CrossRef] [Scilit]
- Bergmann, W.; Feeney, R.J. Contributions to the study of marine products. XXXII. The nucleosides of sponges. I. J. Org. Chem. 1951, 16, 981–987. [Google Scholar] [CrossRef] [Scilit]
- Elion, G.B.; Furman, P.A.; Fyfe, J.A.; de Miranda, P.; Beauchamp, L.; Schaeffer, H.J. Selectivity of action of an antiherpetic agent, 9-(2-hydroxyethoxymethyl) guanine. Proc. Natl. Acad. Sci. USA 1977, 74, 5716–5720. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Privat de Garilhe, M.; de Rudder, J. Effect of 2 arabinose nucleosides on the multiplication of herpes virus and vaccine in cell culture. C. R. Hebd. Seances Acad. Sci. 1964, 259, 2725–2728. [Google Scholar]
- Horwitz, J.P.; Chua, J.; Noel, M. Nucleosides. V. The Monomesylates of 1-(2′-Deoxy-β-D-lyxofuranosyl)thymine1,2. J. Org. Chem. 1964, 29, 2076–2078. [Google Scholar] [CrossRef] [Scilit]
- Nakashima, H.; Matsui, T.; Harada, S.; Kobayashi, N.; Matsuda, A.; Ueda, T.; Yamamoto, N. Inhibition of replication and cytopathic effect of human T cell lymphotropic virus type III/lymphadenopathy-associated virus by 3′-azido-3′-deoxythymidine in vitro. Antimicrob. Agents Chemother. 1986, 30, 933–937. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mitsuya, H.; Weinhold, K.J.; Furman, P.A.; St Clair, M.H.; Lehrman, S.N.; Gallo, R.C.; Bolognesi, D.; Barry, D.W.; Broder, S. 3′-Azido-3′-deoxythymidine (BW A509U): An antiviral agent that inhibits the infectivity and cytopathic effect of human T-lymphotropic virus type III/lymphadenopathy-associated virus in vitro. Proc. Natl. Acad. Sci. USA 1985, 82, 7096–7100. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Muller, W.E.; Sobel, C.; Diehl-Seifert, B.; Maidhof, A.; Schroder, H.C. Influence of the antileukemic and anti-human immunodeficiency virus agent avarol on selected immune responses in vitro and in vivo. Biochem. Pharmacol. 1987, 36, 1489–1494. [Google Scholar] [CrossRef] [Scilit]
- Sakai, R.; Higa, T.; Jefford, C.W.; Bernardinelli, G. Manzamine A, a novel antitumor alkaloid from a sponge. J. Am. Chem. Soc. 1986, 108, 6404–6405. [Google Scholar] [CrossRef] [Scilit]
- Perry, N.B.; Blunt, J.W.; Munro, M.H.G.; Pannell, L.K. Mycalamide A, an antiviral compound from a New Zealand sponge of the genus Mycale. J. Am. Chem. Soc. 1988, 110, 4850–4851. [Google Scholar] [CrossRef] [Scilit]
- Ford, P.W.; Gustafson, K.R.; McKee, T.C.; Shigematsu, N.; Maurizi, L.K.; Pannell, L.K.; Williams, D.E.; de Silva, E.D.; Lassota, P.; Allen, T.M.; et al. Papuamides A−D, HIV-inhibitory and cytotoxic depsipeptides from the sponges Theonella mirabilis and Theonella swinhoei collected in Papua New Guinea. J. Am. Chem. Soc. 1999, 121, 5899–5909. [Google Scholar] [CrossRef] [Scilit]
- Yasuhara-Bell, J.; Lu, Y. Marine compounds and their antiviral activities. Antivir. Res. 2010, 86, 231–240. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Witvrouw, M.; Este, J.A.; Mateu, M.Q.; Reymen, D.; Andrei, G.; Snoeck, R.; Ikeda, S.; Pauwels, R.; Bianchini, N.V.; Desmyter, J.; et al. Activity of a sulfated polysaccharide extracted from the red seaweed Aghardhiella tenera against human immunodeficiency virus and other enveloped viruses. Antivir. Chem. Chemother. 1994, 5, 297–303. [Google Scholar] [CrossRef] [Scilit]
- Nakashima, H.; Kido, Y.; Kobayashi, N.; Motoki, Y.; Neushul, M.; Yamamoto, N. Antiretroviral activity in a marine red alga: Reverse transcriptase inhibition by an aqueous extract of Schizymenia pacifica. J. Cancer Res. Clin. Oncol. 1987, 113, 413–416. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nakashima, H.; Kido, Y.; Kobayashi, N.; Motoki, Y.; Neushul, M.; Yamamoto, N. Purification and characterization of an avian myeloblastosis and human immunodeficiency virus reverse transcriptase inhibitor, sulfated polysaccharides extracted from sea algae. Antivir. Chem. Chemother. 1987, 31, 1524–1528. [Google Scholar] [CrossRef] [Scilit]
- Mitsuya, H.; Looney, D.J.; Kuno, S.; Ueno, R.; Wong-Staal, F.; Broder, S. Dextran sulfate suppression of viruses in the HIV family: Inhibition of virion binding to CD4+ cells. Science 1988, 240, 646–649. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nakashima, H.; Yoshida, O.; Baba, M.; De Clercq, E.; Yamamoto, N. Anti-HIV activity of dextran sulphate as determined under different experimental conditions. Antivir. Res. 1989, 11, 233–246. [Google Scholar] [CrossRef] [Scilit]
- Busso, M.E.; Resnick, L. Anti-human immunodeficiency virus effects of dextran sulfate are strain dependent and synergistic or antagonistic when dextran sulfate is given in combination with dideoxynucleosides. Antimicrob. Agents Chemother. 1990, 34, 1991–1995. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yoshida, T.; Nakashima, H.; Yamamoto, N.; Uryu, T. Anti-AIDS virus activity in vitro of dextran sulfates obtained by sulfation of synthetic and natural dextrans. Polym. J. 1993, 25, 1069–1077. [Google Scholar] [CrossRef] [Scilit]
- Yoshida, O.; Nakashima, H.; Yoshida, T.; Kaneko, Y.; Yamamoto, I.; Matsuzaki, K.; Uryu, T.; Yamamoto, N. Sulfation of the immunomodulating polysaccharide lentinan: A novel strategy for antivirals to human immunodeficiency virus (HIV). Biochem. Pharmacol. 1988, 37, 2887–2891. [Google Scholar] [CrossRef] [Scilit]
- Kaneko, Y.; Yoshida, O.; Nakagawa, R.; Yoshida, T.; Date, M.; Ogihara, S.; Shioya, S.; Matsuzawa, Y.; Nagashima, N.; Irie, Y.; et al. Inhibition of HIV-1 infectivity with curdlan sulfate in vitro. Biochem. Pharmacol. 1990, 39, 793–797. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gao, Y.; Fukuda, A.; Katsuraya, K.; Kaneko, Y.; Mimura, T.; Nakashima, H.; Uryu, T. Synthesis of regioselective substituted curdlan sulfates with medium molecular weights and their specific anti-HIV-1 activities. Macromolecules 1997, 30, 3224–3228. [Google Scholar] [CrossRef] [Scilit]
- Yamamoto, I.; Takayama, K.; Gonda, T.; Matsuzaki, K.; Hatanaka, K.; Yoshida, T.; Uryu, T.; Yoshida, O.; Nakashima, H.; Yamamoto, N.; et al. Synthesis, structure and antiviral activity of sulfates of curdlan and its branched derivatives. Br. Polym. J. 1990, 23, 245–250. [Google Scholar] [CrossRef] [Scilit]
- Koizumi, N.; Sakagami, H.; Utsumi, A.; Fujinaga, S.; Takeda, M.; Asano, K.; Sugawara, I.; Ichikawa, S.; Kondo, H.; Mori, S.; et al. Anti-HIV (human immunodeficiency virus) activity of sulfated paramylon. Antivir. Res. 1993, 21, 1–14. [Google Scholar] [CrossRef] [Scilit]
- Nakashima, H.; Inazawa, K.; Ichiyama, K.; Ito, M.; Ikushima, N.; Shoji, T.; Katsuraya, K.; Uryu, T.; Yamamoto, N.; Juodawlkis, A.S.; et al. Sulfated alkyl oligosaccharides inhibit human immunodeficiency virus in vitro and provide sustained drug levels in mammals. Antivir. Chem. Chemother. 1995, 6, 271–280. [Google Scholar] [CrossRef] [Scilit]
- Witvrouw, M.; De Clercq, E. Sulfated polysaccharides extracted from sea algae as potential antiviral drugs. Gen. Pharmacol. 1997, 29, 497–511. [Google Scholar] [CrossRef] [Scilit]
- Batinic, D.; Robey, F.A. The V3 region of the envelope glycoprotein of human immunodeficiency virus type 1 binds sulfated polysaccharides and CD4-derived synthetic peptides. J. Biol. Chem. 1992, 267, 6664–6671. [Google Scholar] [PubMed]
- Callahan, L.N.; Phelan, M.; Mallinson, M.; Norcross, M.A. Dextran sulfate blocks antibody binding to the principal neutralizing domain of human immunodeficiency virus type 1 without interfering with gp120-CD4 interactions. J. Virol. 1991, 65, 1543–1550. [Google Scholar] [PubMed]
- Mbemba, E.; Chams, V.; Gluckman, J.C.; Klatzmann, D.; Gattegno, L. Molecular interaction between HIV-1 major envelope glycoprotein and dextran sulfate. Biochim. Biophys. Acta 1992, 1138, 62–67. [Google Scholar] [CrossRef] [Scilit]
- Lai, P.K.; Donovan, J.; Takayama, H.; Sakagami, H.; Tanaka, A.; Konno, K.; Nonoyama, M. Modification of human immunodeficiency viral replication by pine cone extracts. AIDS Res. Hum. Retrovir. 1990, 6, 205–217. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nakashima, H.; Murakami, T.; Yamamoto, N.; Naoe, T.; Kawazoe, Y.; Konno, K.; Sakagami, H. Lignified materials as medicinal resources. V. Anti-HIV (human immunodeficiency virus) activity of some synthetic lignins. Chem. Pharm. Bull. 1992, 40, 2102–2105. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mitsuhashi, S.; Kishimoto, T.; Uraki, Y.; Okamoto, T.; Ubukata, M. Low molecular weight lignin suppresses activation of NF-κB and HIV-1 promoter. Bioorg. Med. Chem. 2008, 16, 2645–2650. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fujioka, T.; Kashiwada, Y.; Kilkuskie, R.E.; Cosentino, L.M.; Ballas, L.M.; Jiang, J.B.; Janzen, W.P.; Chen, I.S.; Lee, K.H. Anti-AIDS agents, 11. Betulinic acid and platanic acid as anti-HIV principles from Syzigium claviflorum, and the anti-HIV activity of structurally related triterpenoids. J. Nat. Prod. 1994, 57, 243–247. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kashiwada, Y.; Hashimoto, F.; Cosentino, L.M.; Chen, C.H.; Garrett, P.E.; Lee, K.H. Betulinic acid and dihydrobetulinic acid derivatives as potent anti-HIV agents. J. Med. Chem. 1996, 39, 1016–1017. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kanamoto, T.; Kashiwada, Y.; Kanbara, K.; Gotoh, K.; Yoshimori, M.; Goto, T.; Sano, K.; Nakashima, H. Anti-human immunodeficiency virus activity of YK-FH312 (a betulinic acid derivative), a novel compound blocking viral maturation. Antimicrob. Agents Chemother. 2001, 45, 1225–1230. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, F.; Goila-Gaur, R.; Salzwedel, K.; Kilgore, N.R.; Reddick, M.; Matallana, C.; Castillo, A.; Zoumplis, D.; Martin, D.E.; Orenstein, J.M.; et al. PA-457: A potent HIV inhibitor that disrupts core condensation by targeting a late step in Gag processing. Proc. Natl. Acad. Sci. USA 2003, 100, 13555–13560. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Morimoto, M.; Mori, H.; Otake, T.; Ueba, N.; Kunita, N.; Niwa, M.; Murakami, T.; Iwanaga, S. Inhibitory effect of tachyplesin I on the proliferation of human immunodeficiency virus in vitro. Chemotherapy 1991, 37, 206–211. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Murakami, T.; Niwa, M.; Tokunaga, F.; Miyata, T.; Iwanaga, S. Direct virus inactivation of tachyplesin I and its isopeptides from horseshoe crab hemocytes. Chemotherapy 1991, 37, 327–334. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nakashima, H.; Masuda, M.; Murakami, T.; Koyanagi, Y.; Matsumoto, A.; Fujii, N.; Yamamoto, N. Anti-human immunodeficiency virus activity of a novel synthetic peptide, T22 ([Tyr-5,12, Lys-7]polyphemusin II): A possible inhibitor of virus-cell fusion. Antimicrob. Agents Chemother. 1992, 36, 1249–1255. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Masuda, M.; Nakashima, H.; Ueda, T.; Naba, H.; Ikoma, R.; Otaka, A.; Terakawa, Y.; Tamamura, H.; Ibuka, T.; Murakami, T.; et al. A novel anti-HIV synthetic peptide, T-22 ([Tyr5,12,Lys7]-polyphemusin II). Biochem. Biophys. Res. Commun. 1992, 189, 845–850. [Google Scholar] [CrossRef] [Scilit]
- Arakaki, R.; Tamamura, H.; Premanathan, M.; Kanbara, K.; Ramanan, S.; Mochizuki, K.; Baba, M.; Fujii, N.; Nakashima, H. T134, a small-molecule CXCR4 inhibitor, has no cross-drug resistance with AMD3100, a CXCR4 antagonist with a different structure. J. Virol. 1999, 73, 1719–1723. [Google Scholar] [PubMed]
- Tamamura, H.; Xu, Y.; Hattori, T.; Zhang, X.; Arakaki, R.; Kanbara, K.; Omagari, A.; Otaka, A.; Ibuka, T.; Yamamoto, N.; et al. A low-molecular-weight inhibitor against the chemokine receptor CXCR4: A strong anti-HIV peptide T140. Biochem. Biophys. Res. Commun. 1998, 253, 877–882. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fujii, N.; Oishi, S.; Hiramatsu, K.; Araki, T.; Ueda, S.; Tamamura, H.; Otaka, A.; Kusano, S.; Terakubo, S.; Nakashima, H.; et al. Molecular-size reduction of a potent CXCR4-chemokine antagonist using orthogonal combination of conformation- and sequence-based libraries. Angew. Chem. Int. Ed. Engl. 2003, 42, 3251–3253. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Murakami, T.; Nakajima, T.; Koyanagi, Y.; Tachibana, K.; Fujii, N.; Tamamura, H.; Yoshida, N.; Waki, M.; Matsumoto, A.; Yoshie, O.; et al. A small molecule CXCR4 inhibitor that blocks T cell line-tropic HIV-1 infection. J. Exp. Med. 1997, 186, 1389–1393. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xu, Y.; Tamamura, H.; Arakaki, R.; Nakashima, H.; Zhang, X.; Fujii, N.; Uchiyama, T.; Hattori, T. Marked increase in anti-HIV activity, as well as inhibitory activity against HIV entry mediated by CXCR4, linked to enhancement of the binding ability of tachyplesin analogs to CXCR4. AIDS Res. Hum. Retrovir. 1999, 15, 419–427. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Murakami, T.; Zhang, T.Y.; Koyanagi, Y.; Tanaka, Y.; Kim, J.; Suzuki, Y.; Minoguchi, S.; Tamamura, H.; Waki, M.; Matsumoto, A.; et al. Inhibitory mechanism of the CXCR4 antagonist T22 against human immunodeficiency virus type 1 infection. J. Virol. 1999, 73, 7489–7496. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ohashi, N.; Tamamura, H. Peptide-derived mid-sized anti-HIV agents. Amino Acids Pept. Proteins 2017, 41, 1–29. [Google Scholar] [CrossRef] [Scilit]
- Ma, X.; Li, L.; Zhu, T.; Ba, M.; Li, G.; Gu, Q.; Guo, Y.; Li, D. Phenylspirodrimanes with anti-HIV activity from the sponge-derived fungus Stachybotrys chartarum MXH-X73. J. Nat. Prod. 2013, 76, 2298–2306. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Vidal, V.; Potterat, O.; Louvel, S.; Hamy, F.; Mojarrab, M.; Sanglier, J.J.; Klimkait, T.; Hamburger, M. Library-based discovery and characterization of daphnane diterpenes as potent and selective HIV inhibitors in Daphne gnidium. J. Nat. Prod. 2012, 75, 414–419. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tietjen, I.; Ntie-Kang, F.; Mwimanzi, P.; Onguene, P.A.; Scull, M.A.; Idowu, T.O.; Ogundaini, A.O.; Meva’a, L.M.; Abegaz, B.M.; Rice, C.M.; et al. Screening of the Pan-African natural product library identifies ixoratannin A-2 and boldine as novel HIV-1 inhibitors. PLoS ONE 2015, 10, e0121099. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mori, T.; O’Keefe, B.R.; Sowder, R.C., 2nd; Bringans, S.; Gardella, R.; Berg, S.; Cochran, P.; Turpin, J.A.; Buckheit, R.W., Jr.; McMahon, J.B.; et al. Isolation and characterization of griffithsin, a novel HIV-inactivating protein, from the red alga Griffithsia sp. J. Biol. Chem. 2005, 280, 9345–9353. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- O’Keefe, B.R.; Vojdani, F.; Buffa, V.; Shattock, R.J.; Montefiori, D.C.; Bakke, J.; Mirsalis, J.; d’Andrea, A.L.; Hume, S.D.; Bratcher, B.; et al. Scaleable manufacture of HIV-1 entry inhibitor griffithsin and validation of its safety and efficacy as a topical microbicide component. Proc. Natl. Acad. Sci. USA 2009, 106, 6099–6104. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lai, W.; Huang, L.; Zhu, L.; Ferrari, G.; Chan, C.; Li, W.; Lee, K.H.; Chen, C.H. Gnidimacrin, a Potent Anti-HIV Diterpene, Can Eliminate Latent HIV-1 Ex Vivo by Activation of Protein Kinase C beta. J. Med. Chem. 2015, 58, 8638–8646. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hassan, S.T.; Masarcikova, R.; Berchova, K. Bioactive natural products with anti-herpes simplex virus properties. J. Pharm. Pharmacol. 2015, 67, 1325–1336. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Vo, T.S.; Ngo, D.H.; Ta, Q.V.; Kim, S.K. Marine organisms as a therapeutic source against herpes simplex virus infection. Eur. J. Pharm. Sci. 2011, 44, 11–20. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mandal, P.; Pujol, C.A.; Damonte, E.B.; Ghosh, T.; Ray, B. Xylans from Scinaia hatei: Structural features, sulfation and anti-HSV activity. Int. J. Biol. Macromol. 2010, 46, 173–178. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Duarte, M.E.; Noseda, D.G.; Noseda, M.D.; Tulio, S.; Pujol, C.A.; Damonte, E.B. Inhibitory effect of sulfated galactans from the marine alga Bostrychia montagnei on herpes simplex virus replication in vitro. Phytomedicine 2001, 8, 53–58. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Talarico, L.B.; Zibetti, R.G.; Faria, P.C.; Scolaro, L.A.; Duarte, M.E.; Noseda, M.D.; Pujol, C.A.; Damonte, E.B. Anti-herpes simplex virus activity of sulfated galactans from the red seaweeds Gymnogongrus griffithsiae and Cryptonemia crenulata. Int. J. Biol. Macromol. 2004, 34, 63–71. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Park, H.J.; Kurokawa, M.; Shiraki, K.; Nakamura, N.; Choi, J.S.; Hattori, M. Antiviral activity of the marine alga Symphyocladia latiuscula against herpes simplex virus (HSV-1) in vitro and its therapeutic efficacy against HSV-1 infection in mice. Biol. Pharm. Bull. 2005, 28, 2258–2262. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pifarre, M.P.; Berra, A.; Coto, C.E.; Alche, L.E. Therapeutic action of meliacine, a plant-derived antiviral, on HSV-induced ocular disease in mice. Exp. Eye Res. 2002, 75, 327–334. [Google Scholar] [CrossRef] [PubMed]
- Petrera, E.; Coto, C.E. Therapeutic effect of meliacine, an antiviral derived from Melia azedarach L., in mice genital herpetic infection. Phytother. Res. 2009, 23, 1771–1777. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hayashi, T.; Kawasaki, M.; Miwa, Y.; Taga, T.; Morita, N. Antiviral agents of plant origin. III. Scopadulin, a novel tetracyclic diterpene from Scoparia dulcis L. Chem. Pharm. Bull. 1990, 38, 945–947. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hayashi, T.; Hayashi, K.; Maeda, M.; Kojima, I. Calcium spirulan, an inhibitor of enveloped virus replication, from a blue-green alga Spirulina platensis. J. Nat. Prod. 1996, 59, 83–87. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lee, J.B.; Hayashi, K.; Hashimoto, M.; Nakano, T.; Hayashi, T. Novel antiviral fucoidan from sporophyll of Undaria pinnatifida (Mekabu). Chem. Pharm. Bull. 2004, 52, 1091–1094. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kanekiyo, K.; Lee, J.B.; Hayashi, K.; Takenaka, H.; Hayakawa, Y.; Endo, S.; Hayashi, T. Isolation of an antiviral polysaccharide, nostoflan, from a terrestrial cyanobacterium, Nostoc flagelliforme. J. Nat. Prod. 2005, 68, 1037–1041. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Docherty, J.J.; Sweet, T.J.; Bailey, E.; Faith, S.A.; Booth, T. Resveratrol inhibition of varicella-zoster virus replication in vitro. Antivir. Res. 2006, 72, 171–177. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- De Leo, A.; Arena, G.; Lacanna, E.; Oliviero, G.; Colavita, F.; Mattia, E. Resveratrol inhibits Epstein Barr Virus lytic cycle in Burkitt’s lymphoma cells by affecting multiple molecular targets. Antivir. Res. 2012, 96, 196–202. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Evers, D.L.; Wang, X.; Huong, S.M.; Huang, D.Y.; Huang, E.S. 3,4′,5-Trihydroxy-trans-stilbene (resveratrol) inhibits human cytomegalovirus replication and virus-induced cellular signaling. Antivir. Res. 2004, 63, 85–95. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dyson, O.F.; Walker, L.R.; Whitehouse, A.; Cook, P.P.; Akula, S.M. Resveratrol inhibits KSHV reactivation by lowering the levels of cellular EGR-1. PLoS ONE 2012, 7, e33364. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ourth, D.D. Susceptibility in vitro of Epstein-Barr Virus to myristoylated-peptide. Peptides 2010, 31, 1409–1411. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Prusty, B.K.; Das, B.C. Constitutive activation of transcription factor AP-1 in cervical cancer and suppression of human papillomavirus (HPV) transcription and AP-1 activity in HeLa cells by curcumin. Int. J. Cancer 2005, 113, 951–960. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Slater, M.J.; Cockerill, S.; Baxter, R.; Bonser, R.W.; Gohil, K.; Gowrie, C.; Robinson, J.E.; Littler, E.; Parry, N.; Randall, R.; et al. Indolocarbazoles: Potent, selective inhibitors of human cytomegalovirus replication. Bioorg. Med. Chem. 1999, 7, 1067–1074. [Google Scholar] [CrossRef] [Scilit]
- Nixon, B.; Stefanidou, M.; Mesquita, P.M.; Fakioglu, E.; Segarra, T.; Rohan, L.; Halford, W.; Palmer, K.E.; Herold, B.C. Griffithsin protects mice from genital herpes by preventing cell-to-cell spread. J. Virol. 2013, 87, 6257–6269. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Levendosky, K.; Mizenina, O.; Martinelli, E.; Jean-Pierre, N.; Kizima, L.; Rodriguez, A.; Kleinbeck, K.; Bonnaire, T.; Robbiani, M.; Zydowsky, T.M.; et al. Griffithsin and Carrageenan Combination To Target Herpes Simplex Virus 2 and Human Papillomavirus. Antimicrob. Agents Chemother. 2015, 59, 7290–7298. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Takebe, Y.; Saucedo, C.J.; Lund, G.; Uenishi, R.; Hase, S.; Tsuchiura, T.; Kneteman, N.; Ramessar, K.; Tyrrell, D.L.; Shirakura, M.; et al. Antiviral lectins from red and blue-green algae show potent in vitro and in vivo activity against hepatitis C virus. PLoS ONE 2013, 8, e64449. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Buck, C.B.; Thompson, C.D.; Roberts, J.N.; Muller, M.; Lowy, D.R.; Schiller, J.T. Carrageenan is a potent inhibitor of papillomavirus infection. PLoS Pathog. 2006, 2, e69. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Roberts, J.N.; Buck, C.B.; Thompson, C.D.; Kines, R.; Bernardo, M.; Choyke, P.L.; Lowy, D.R.; Schiller, J.T. Genital transmission of HPV in a mouse model is potentiated by nonoxynol-9 and inhibited by carrageenan. Nat. Med. 2007, 13, 857–861. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Marais, D.; Gawarecki, D.; Allan, B.; Ahmed, K.; Altini, L.; Cassim, N.; Gopolang, F.; Hoffman, M.; Ramjee, G.; Williamson, A.L. The effectiveness of Carraguard, a vaginal microbicide, in protecting women against high-risk human papillomavirus infection. Antivir. Ther. 2011, 16, 1219–1226. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Malonza, I.M.; Mirembe, F.; Nakabiito, C.; Odusoga, L.O.; Osinupebi, O.A.; Hazari, K.; Chitlange, S.; Ali, M.M.; Callahan, M.; Van Damme, L. Expanded Phase I safety and acceptability study of 6% cellulose sulfate vaginal gel. AIDS 2005, 19, 2157–2163. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- El-Sadr, W.M.; Mayer, K.H.; Maslankowski, L.; Hoesley, C.; Justman, J.; Gai, F.; Mauck, C.; Absalon, J.; Morrow, K.; Masse, B.; et al. Safety and acceptability of cellulose sulfate as a vaginal microbicide in HIV-infected women. AIDS 2006, 20, 1109–1116. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Van Damme, L.; Govinden, R.; Mirembe, F.M.; Guedou, F.; Solomon, S.; Becker, M.L.; Pradeep, B.S.; Krishnan, A.K.; Alary, M.; Pande, B.; et al. Lack of effectiveness of cellulose sulfate gel for the prevention of vaginal HIV transmission. N. Engl. J. Med. 2008, 359, 463–472. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Derby, N.; Lal, M.; Aravantinou, M.; Kizima, L.; Barnable, P.; Rodriguez, A.; Lai, M.; Wesenberg, A.; Ugaonkar, S.; Levendosky, K.; et al. Griffithsin carrageenan fast dissolving inserts prevent SHIV HSV-2 and HPV infections in vivo. Nat. Commun. 2018, 9, 3881. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Punfa, W.; Yodkeeree, S.; Pitchakarn, P.; Ampasavate, C.; Limtrakul, P. Enhancement of cellular uptake and cytotoxicity of curcumin-loaded PLGA nanoparticles by conjugation with anti-P-glycoprotein in drug resistance cancer cells. Acta Pharmacol. Sin. 2012, 33, 823–831. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zaman, M.S.; Chauhan, N.; Yallapu, M.M.; Gara, R.K.; Maher, D.M.; Kumari, S.; Sikander, M.; Khan, S.; Zafar, N.; Jaggi, M.; et al. Curcumin Nanoformulation for Cervical Cancer Treatment. Sci. Rep. 2016, 6, 20051. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gong, C.; Wu, Q.; Wang, Y.; Zhang, D.; Luo, F.; Zhao, X.; Wei, Y.; Qian, Z. A biodegradable hydrogel system containing curcumin encapsulated in micelles for cutaneous wound healing. Biomaterials 2013, 34, 6377–6387. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, G.; Li, J.; Cai, Y.; Zhan, J.; Gao, J.; Song, M.; Shi, Y.; Yang, Z. A Glycyrrhetinic Acid-Modified Curcumin Supramolecular Hydrogel for liver tumor targeting therapy. Sci. Rep. 2017, 7, 44210. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Porter, S.R.; Al-Johani, K.; Fedele, S.; Moles, D.R. Randomised controlled trial of the efficacy of HybenX in the symptomatic treatment of recurrent aphthous stomatitis. Oral Dis. 2009, 15, 155–161. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nibali, L.; Atkinson, C.; Griffiths, P.; Darbar, U.; Rakmanee, T.; Suvan, J.; Donos, N. Low prevalence of subgingival viruses in periodontitis patients. J. Clin. Periodontol. 2009, 36, 928–932. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Agut, H.; Bonnafous, P.; Gautheret-Dejean, A. Laboratory and clinical aspects of human herpesvirus 6 infections. Clin. Microbiol. Rev. 2015, 28, 313–335. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Asai, D.; Kanamoto, T.; Takenaga, M.; Nakashima, H. In situ depot formation of anti-HIV fusion-inhibitor peptide in recombinant protein polymer hydrogel. Acta Biomater. 2017, 64, 116–125. [Google Scholar] [CrossRef] [Scilit] [PubMed]

© 2018 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (http://creativecommons.org/licenses/by/4.0/).