


Abstract
Salmonella remains a leading cause of foodborne illness worldwide, with non-typhoidal Salmonella (NTS) responsible for an estimated 93.8 million infections and substantial global morbidity and mortality. This review synthesizes current evidence on the epidemiology, molecular pathogenesis, and prevention of both typhoidal and nontyphoidal Salmonella, with emphasis on emerging challenges in disease control. We highlight key virulence mechanisms, including Salmonella pathogenicity islands and Type III secretion systems, that mediate host cell invasion, intracellular survival, and immune modulation, alongside differences in host adaptation, reservoirs, and clinical outcomes between major serotypes. Epidemiological synthesis demonstrates marked geographic variability in disease burden, driven by underreporting, limited diagnostic capacity, and social determinants of health, with particularly high mortality from invasive NTS (iNTS) disease in sub-Saharan Africa. This review further identifies major challenges, including the global rise of multidrug-resistant Salmonella lineages, the emergence of high-risk serotypes such as monophasic S. Typhimurium and S. Infantis, and the increasing complexity of transmission across the farm-to-fork continuum. While advances in whole genome sequencing and integrated surveillance platforms (e.g., PulseNet and GenomeTrakr) have improved outbreak detection and source attribution, gaps in cross-sector coordination persist. Collectively, the evidence underscores the need for integrated One Health approaches that link human, animal, and environmental systems, alongside strengthened surveillance, targeted prevention strategies, and antimicrobial stewardship. Advances in vaccination, including licensed typhoidal vaccines such as Ty21a and Vi polysaccharide, and conjugate vaccines, as well as emerging live attenuated and glycoconjugate candidates targeting NTS, represent promising strategies for reducing the global burden of Salmonella infections. Future efforts should focus on improving global surveillance harmonization, addressing environmental and climate-related drivers of transmission, and advancing vaccine development and implementation.
1. Introduction
Salmonella is a Gram-negative, facultative intracellular, rod-shaped and non-spore-forming member of the Enterobacteriaceae family [1]. The bacterial genus Salmonella is divided into two species, Salmonella bongori (S. bongori) and Salmonella enterica (S. enterica). S. enterica consists of six subspecies: enterica, salamae, arizona, diarizonae, indica and houtenae of which S. enterica subspecies enterica consists of more than 2400 serotypes [2,3]. Typically, Salmonella serotypes are classified into typhoidal (primarily S. enterica subspecies enterica serovar Typhi) and non-typhoidal serotypes (NTS) (like S. Enteritidis, S. Typhimurium and S. Newport) [4,5,6]. Typhoidal Salmonella infections are characterized by typhoid fever and invasive disease, while NTS infections mostly present with self-limiting gastrointestinal disease, which may lead to hospitalization or death. In sub-Saharan Africa, NTS species are known to cause invasive disease (iNTS) that can present as bacteremia with mortality rates approaching 20% [7,8]. Traditionally, NTS infections have been attributed to the consumption of poultry meat and eggs. However, in recent years, fresh produce and other associated food products have been the cause of numerous food-borne outbreaks [9,10]. The global burden for NTS is in the millions, leading to a significant number of deaths, hospitalizations, and massive costs to the health care system [11,12]. Despite increased global surveillance, enhanced detection, and consumer education, NTS remains a public health concern [13].
Given the complexity and continued global burden of Salmonella infections, this review aims to synthesize current knowledge on key aspects of Salmonella biology and public health impact. Specifically, we summarize the epidemiology and global burden of typhoidal and NTS infections and highlight major virulence mechanisms contributing to pathogenesis. We further discuss emerging public health challenges, including the global rise in antimicrobial resistance, the emergence of high-risk serotypes, and evolving transmission dynamics across the farm-to-fork continuum.
In addition, this review emphasizes a One Health approach by integrating human, animal, and environmental perspectives to better understand Salmonella transmission and persistence across interconnected systems. A focused case study examining Salmonella transmission and control in pork production systems is included to illustrate the application of a One Health, farm-to-fork framework in a high-risk food production environment. Surveillance and control strategies are then evaluated in the context of current advances in molecular detection, genomic epidemiology, and integrated monitoring platforms. Prevention strategies, including food safety interventions and vaccination approaches, are also reviewed. Collectively, these findings highlight the need for comprehensive and integrated One Health approaches to curb the continued impact of NTS worldwide.
2. Global Epidemiological Trends
2.1. Salmonella Incidence
2.1.1. Global Incidence and Burden
NTS cases have continued to steadily increase, with a current global case estimate of 93.8 million. Of those cases, there have been 155 thousand reported deaths [14,15]. In the United States, it is estimated that there have been over 1.35 million NTS cases, 26,500 hospitalizations, and 420 deaths [16]. In 2024, salmonellosis was the second most reported zoonotic disease in Europe, with 18.6 confirmed cases per 100,000 people [17]. These estimates differ depending on the region’s surveillance methodology, with some regions only reporting laboratory-confirmed cases (European Union, EU) and others adjusting based on surveys and statistical methods to account for underdiagnosis (U.S.) [18]. Additionally, disease burden is often underestimated in many developing countries due to limitations in diagnostic capacity, including insufficient microbiology laboratories, technicians, and surveillance frameworks. In many African and South American nations, it is estimated that only 1–10% of cases are reported [19]. With many cases being self-limiting or subclinical, they often go unreported when individuals do not seek medical care [20].
Geographic variability in salmonellosis incidence is influenced by a complex interplay of structural, environmental, and healthcare-related factors [21]. Differences in surveillance systems and reporting capacity may contribute to underestimation of disease burden in certain regions, particularly in medically underserved areas with limited access to healthcare and diagnostic services. Environmental and agricultural characteristics also play a role; for example, counties with greater agricultural activity, increased wetland coverage, and impaired surface waterways have been associated with higher salmonellosis incidence. Evidence from a 22-year analysis of Laboratory Enteric Disease Surveillance (LEDS) data (1997–2019), using a counterfactual random forest analysis, further demonstrates that structural inequities, social determinants of health, and environmental factors, including extreme weather, contribute to disparities in salmonellosis incidence across U.S. counties [21]. Additionally, these factors may influence both true disease burden and reporting patterns. These findings underscore the importance of targeted public health interventions, including improved surveillance, enhanced food safety practices, and community-specific prevention strategies.
2.1.2. High-Risk Regions and Vulnerable Populations
Preventing foodborne salmonellosis relies on avoiding cross-contamination and ensuring proper handling of food. This leads to significant variation across regions depending on agricultural practices and food safety regulations. Given the disease’s fecal–oral route of disease transmission, overcrowding, poor water sanitation, and poor hygiene infrastructure contribute to a higher disease burden, leaving low-resource settings particularly vulnerable. This is reflected in regions such as Sub-Saharan Africa, where the death rate for iNTS is 15–25% [13]. Additionally, host risk factors for contracting NTS include advanced age, young children, severe malnourishment, and immunocompromised individuals. Interestingly, there is a particularly significant association between individuals with HIV and their susceptibility to iNTS due to the vital role of Th17 and CD4 T cells in combating Salmonella infection [22]. Of the 77,500 deaths in sub-Saharan Africa, 18,400 of those cases were linked to HIV coinfection [9,23].
2.2. Trends in Serotypes
2.2.1. Dominant NTS Serotypes
Within the S. enterica species, over 2400 non-typhoidal serotypes have been identified worldwide and are classified based on their surface antigens and reactions with antibodies [3,24]. The distribution and prevalence of these serotypes vary by region (Table 1); however, S. Typhimurium and S. Enteritidis have remained among the dominant serotypes, accounting for over 40% of the total outbreaks in the U.S. [12]. The European Union (EU) reported that the top NTS serotypes from 2018–2021 included S. Typhimurium, S. Enteritidis, monophasic variant of S. Typhimurium (MVST), S. Infantis, and S. Derby. Moreover, S. Enteritidis has remained the dominant EU NTS serotype for decades and has steadily increased from 61.6% to 64.6% of reported cases [25]. Similarly, the aforementioned serotypes have also been reported as the most common serotypes in Africa [26,27]. However, the strain most strongly associated with the region’s high burden of invasive disease is S. Typhimurium sequence type ST313, with a large proportion characterized by multidrug resistance (MDR) [27].
Table 1.
Summary of dominant and emerging NTS Salmonella strains.
2.2.2. Emerging and Re-Emerging Serotypes Worldwide
Aside from the dominant serotypes, several others have emerged and re-emerged, including S. Infantis and the MVST. Among these, MVST has been at the forefront of emerging serotypes and is most commonly associated with pork products [28]. It first emerged in Portugal in the 1980s and has since increased in prevalence across the United States and Europe [28]. In 2021, MVST was the most frequently reported serotype in Italy, with 1115 reported cases [28]. Likewise, in Europe, reported MVST cases increased from 1738 in 2023 to 3860 in 2024, making this serotype the third most commonly reported serotype after S. Enteritidis [17]. Another emerging serotype is S. Infantis; however, unlike MVST, it is predominantly associated with poultry. It is considered the fourth most common serotype in the EU and is frequently associated with multidrug resistance through its megaplasmid known as plasmid of emerging S. Infantis (pESI) [29]. It has also recently emerged in the U.S. and Latin America. In a global systematic review (1979–2021), 42.9% of the reported S. Infantis isolates were found in the Americas, while 29.8% were found in the EU [30]. More recently, phylogenetic analyses have demonstrated that S. Infantis forms a monophyletic lineage that likely originated in West Asia around 1990, followed by spread to Europe, South America, and North America. It has continuously developed more resistance through the expansion of the American sublineage, which has disseminated across all continents. This sublineage includes the extended-spectrum β-lactamase (ESBL)-encoding blaCTX-M-65 gene, which has further limited treatment options for invasive infections [31].
2.3. Outbreak Patterns
2.3.1. Foodborne Versus Non-Foodborne Outbreaks
Recent analyses of outbreak surveillance data from 1998–2022 released by the Interagency Food Safety Analytics Collaboration (IFSAC) state that approximately 75% of human Salmonella infections are attributable to foodborne transmission [32]. Some common infected sources from recent multistate outbreaks from 2024–2025 (Table 2) include backyard poultry (1029 total cases; 470 in 2024 and 559 in 2025, an 18.9% increase), eggs (227 total cases; 93 in 2024 and 134 in 2025, a 44.1% increase), and cucumbers (620 total cases; 551 in 2024 and 69 in 2025), all of which may become contaminated at various stages of farming, processing, or food handling. In addition, a charcuterie meat-associated outbreak reported in 2024 resulted in 104 cases [10,33,34].
Table 2.
Foodborne and Non-Foodborne Salmonella Transmission Types: Reported Case Counts & Hospitalizations from Recent CDC Multistate Outbreaks (2024–2025).
Common sources for non-foodborne transmissions that are relatively rare but still important include contact with animal feces and reptiles such as pet bearded dragons (26 cases), geckos (49 cases), and small turtles (63 cases) [33]. Other non-foodborne exposures include contaminated water sources and interpersonal transmission, especially in settings such as petting zoos, farms, fairs, schools, and daycares [35]. According to CDC’s Animal Contact Outbreak Surveillance System (ACOSS) data from 2009–2021 (Table 3), 545 enteric disease outbreaks associated with direct or indirect animal contact in the United States resulted in 14,215 illnesses, with Salmonella identified as one of the most commonly reported pathogens. Among these outbreaks, 417 had a single reported location of exposure with 6354 illnesses. Of those single-location outbreaks, the most frequently reported settings were private homes (168 outbreaks), public farms or dairies (89 outbreaks), festivals or fairs (36 outbreaks), petting zoos (28 outbreaks), and institutional settings such as schools and daycares (28 outbreaks) [36]. As foodborne and non-foodborne outbreaks intersect with distribution systems that span multiple jurisdictions, the critical role of multistate and multi-country outbreak investigation processes are highlighted.
Table 3.
Single-Location Animal Contact Outbreaks and Associated Illnesses: ACOSS, US 2009–2021.
2.3.2. Multistate/Multi-Country Outbreak Investigations
Stages of multistate outbreak investigation are closely parallel to multi-country outbreak investigation frameworks with both grounded in a shared, systematic epidemiologic methodology (Figure 1). The process begins with confirmation that an outbreak is occurring, characterized by an unusual increase in linked cases, followed by verification of the causative agent [37,38]. Standardized case definitions, also known as case count, are developed and refined to clearly specify which individuals meet the criteria for case inclusion [39]. Using this case definition, investigators conduct active case and contact finding through medical records, patient interviews, and fieldwork, and analyze the resulting data by time, place, and person using epidemic curves, geographic mapping, and demographic characteristics to identify patterns of illness [40]. These descriptive findings inform hypothesis generation regarding possible sources of exposure and modes of transmission, which are subsequently evaluated using methods such as case–control or cohort studies [41]. Once a likely source is identified, both frameworks incorporate traceback investigations, laboratory, and environmental testing to determine where contamination may have occurred [40]. Finally, control measures are implemented to limit further transmission, and findings are communicated to public health authorities, regulatory food and veterinary authorities, and the public [42].
Figure 1.
Stages of Outbreak Investigation.
2.3.3. Role of Globalization, Travel, and Trade
Globalization has changed food systems through centralized production, international ingredient sourcing, and integrated supply chains, creating the structural framework that enables Salmonella to spread beyond local boundaries [43]. Within this structural framework, trade acts as the primary mechanism for dissemination, with evidence from multiple regions, including the United States, China, and Mexico, demonstrating a correlation between increased import–export movement and rising salmonellosis incidence [44,45,46]. International travel further contributes to Salmonella outbreaks, with 19% of cases being identified as a major risk factor for high antimicrobial resistance infections, complicating clinical treatment and management [47,48]. A 2019–2023 systematic review that documented multiple disease outbreaks on travel cruise ships, where shared food sources, close living arrangements, and frequent port contact occurred, reported Salmonella to be at least one causative agent, as well as Norovirus, Shigella, and other pathogens [49]. As the globalization of food systems, trade, and travel continues to contribute to the global Salmonella burden, it stresses the importance of continual technological advancements in surveillance systems and collaboration among national and international organizations to link cases across borders.
2.4. Surveillance Advances
2.4.1. Whole Genome Sequencing (WGS) and Genomic Epidemiology
A critical step in routine outbreak investigation and food quality control includes the rapid yet sensitive detection of different Salmonella serotypes. Whole genome sequencing (WGS) has substantially reshaped surveillance, surpassing other traditional, time-consuming phenotyping methods that can take up to days and weeks [50]. WGS allows for rapid high-resolution tracking and source attribution between closely related isolates in a few hours, with reported overall accuracies >90% and especially strong predictive measures for poultry-associated isolates [51]. The identification of new, emerging, or antimicrobial resistance strains has also been enhanced, supporting more targeted clinical interventions [52]. Adoption of WGS by public health agencies has been a gold standard for many years to build databases that allow for real-time tracking of Salmonella infections and collaboration between national and international surveillance platforms, reducing the time needed to investigate outbreaks and enabling faster food recalls and public health decision making [53,54].
2.4.2. Integration of National and International Surveillance Platforms (PulseNet, GenomeTrakr, ECDC, WHO)
Although genomic sequencing provides high-resolution differentiation among Salmonella serotypes, its public health impact depends on coordinated international surveillance systems that can translate genomic data into outbreak detection, source attribution, and timely intervention. In the United States, PulseNet, coordinated by the CDC, uses whole-genome sequencing for high-resolution comparison of clinical isolates and real-time outbreak detection, while GenomeTrakr, led by the FDA, complements this effort by linking genomic data from food and environmental isolates to support source tracking and regulatory action [53,55,56]. Beyond these U.S.-based systems, the European Centre for Disease Prevention and Control (ECDC) and the World Health Organization (WHO) play critical roles in expanding surveillance capacity through a broader One Health framework. In the European Union, the ECDC works closely with the European Food Safety Authority (EFSA) under Directive 2003/99/EC to support harmonized zoonotic and foodborne disease surveillance across Member States [17]. Human case data are reported through EpiPulse Cases, while Epi-Pulse enables real-time communication on emerging clusters, and joint ECDC-EFSA molecular databases integrate whole-genome sequencing and other typing methods across human, animal, food, and environmental sources to improve early detection of multi-country outbreaks and source attribution [57,58]. When such outbreaks are identified, ECDC and EFSA issue Rapid Outbreak Assessments to guide interventions and inform policymakers. At the global level, the WHO, in partnership with the Food and Agriculture Organization through the International Food Safety Authorities Network (INFOSAN), provides the primary platform for international food safety communication and emergency coordination, linking hundreds of members across 188 Member States and facilitating rapid alerts when contaminated food enters global trade. INFOSAN also supports emergency preparedness under the International Health Regulations and maintains links with regional alert systems and laboratory networks, including PulseNet International, helping translate laboratory findings into recalls, trade actions, and broader public health responses [53,57,58]. Together, these systems strengthen global Salmonella surveillance by integrating human, food, animal, and environmental data, improving detection of multi-state and multi-country outbreaks, and ensuring that endemic regional threats are elevated to international public health attention.
3. Molecular Biology and Pathogenesis Updates
3.1. Virulence Factor Insights
3.1.1. Salmonella Pathogenicity Islands and Type 3 Secretion Systems
With the bacteria’s widespread impact, the Salmonella Pathogenicity Islands (SPI) and the Type 3 Secretion System (T3SS) are among Salmonella’s major virulence factors, of which SPI-1 and SPI-2 are noteworthy, both of which encode for their respective injectisomes and effector proteins. T3SS-1, encoded by SPI-1, is primarily activated upon contact with the target cell membrane, facilitating the release of effector proteins leading to invasion of the host epithelial cell [59,60,61]. T3SS-2, encoded by SPI-2, plays a major role in intracellular survival via its actions on Salmonella-containing vacuoles (SCVs) [59,60,61,62]. Human-derived intestinal epithelial cells cultured with Salmonella strains lacking SPI-1 demonstrated a statistically significant decrease in both the mean vacuolar load and percentage of infected cells compared to the wild-type (WT) strain [62]. As for SPI-2, the virulence factor enables the bacteria to survive in the host cells and systematically spread into other organs [59,60,61]. NTS clinical isolates from 200 Saudi Arabian patients in one study detected both SPIs, with 99% being positive for SPI-1 and 84.5% for SPI-2, indicating the epidemiologic importance of these genes [63]. However, SPI-1’s absence in certain human clinical strains (e.g., S. Senftenberg) does suggest other mechanisms that still lead to gastroenteritis [64].
3.1.2. Adhesion, Invasion, Intracellular Survival Mechanisms
One mechanism for Salmonella adhesion is through its fimbriae, as they enable the pathogen to attach onto target cells by interacting with the intestinal epithelial cells’ extracellular matrix (ECM) [65,66]. Salmonella also utilizes non-fimbrial adhesins to latch onto enterocytes, with SiiE being notable [67]. Facilitated by a type I secretion system (T1SS) derived from SPI-4, the adhesin binds to cell surface structures consisting of N-acetylglucosamine and α2-3-linked sialic acid [67].
Regarding invasion, Salmonella has a plethora of strategies to enter the host cells. The trigger mechanism—mediated by the T3SS-1 effectors—uses multiple proteins to significantly promote and stabilize actin polymerization, resulting in membrane ruffling and bacterial entry [61,66,68,69]. Another method is the zipper mechanism, which utilizes direct contact between Salmonella’s Rck and PagN ligands and host cell surface receptors to invoke bacterial internalization [66,68,69]. Other invasion methodology includes the bacteria interacting with microfold (M) cells to undergo transcytosis or hijacking phagocytic cells [60,66,69]. As for Salmonella’s intracellular survival, the SCV is a notable component as it shields the bacteria from the host’s defenses by preventing lysosomal fusion [59,60,65].
3.2. Host–Pathogen Interactions
3.2.1. Interaction with Intestinal Epithelium, Immune Evasion
As previously stated, the trigger mechanism, mediated by T3SS-1, kickstarts the process with multiple effector proteins, including SipA, SipC, SopB, SopE, and SopE2 [61,66,68]. SipA and SipC are involved in modifying host cells’ cytoskeleton by stabilizing actin via direct binding, with the former further involved by inhibiting actin depolymerization [60,61,66,68,69]. SopB, SopE, and SopE2 promote Salmonella invasion by inducing actin remodeling via Rho GTPase family proteins [61,66,68]. The zipper mechanism utilizes the direct binding of Salmonella’s Rck and PagN ligands to EGFR and proteoglycan/β-1 integrin, respectively [66,68,69]. Both ligand–receptor interactions ultimately result in actin polymerization, enabling bacterial entry into the intestinal epithelium with minor membrane ruffling [66,68,69]. Another entrance for Salmonella is M cells, with S. Typhimurium particularly converting follicle-associated epithelial cells into M cells via SopB and exploiting them with ligand–receptor interactions such as transcytosis via FimH/Glycoprotein 2 (GP2) [66,68,69]. Other opportunities involve specific phagocytes such as CXCR1+ dendritic cells (DCs) and macrophages, with the bacteria exploiting these cells to cross over the intestinal barrier [61,66,69].
Additionally, Salmonella can induce an M2 phenotype in infected macrophages, with the SteE effector driving the process by promoting lower NLRP3 inflammasome activity and allowing for greater survivability [69,70,71]. SpvD can also induce an anti-inflammatory state among the immune cells by blocking the NF-κB mechanism [60,66,70]. SteD is another factor in circumventing host defenses by targeting antigen presentation on major histocompatibility complex (MHC)-II, resulting in less CD4+ T cell activation and ultimately immunosuppression [70,72]. Other notable agents involved in immune evasion are SpvC and AvrA, which target MAPK and JNK pathways, respectively, to promote an anti-inflammatory environment [60,66,70,71]. Recent genomic data of 223 clinical Salmonella isolates indicates that within-host variation in both virulence and resistance genes (e.g., emrB, sseB) could ultimately shape the bacteria’s pathogenesis and treatment response [73].
3.2.2. Differences in Virulence Among Major Serotypes
Major Salmonella serotypes share a conserved core virulence for epithelial invasion and intracellular survival, but they differ in host adaptation, immune evasion, and accessory genomes, producing substantially different clinical outcomes [74]. According to the U.S. FoodNet data (1996–2006), serotypes differed substantially in invasiveness and clinical severity: S. Dublin and S. Choleraesuis stood out with very high proportions of invasive infections (blood isolates) and higher hospitalization rates (64% and 57%, respectively) compared with other common gastroenteritis-associated serotypes like S. Enteritidis and S. Typhimurium [74]. Moreover, S. Dublin is disproportionately associated with bloodstream infection, longer hospital stays, and death, characterizing it as a much more invasive serotype [75].
Mechanistically, the major subtypes are divided into typhoidal serotypes (including S. Typhi and S. Paratyphi) and non-typhoidal serotypes (including S. Typhimurium, S. Enteritidis, S. Dublin, S. Choleraesuis, S. Heidelberg, S. Newport). Typhoidal strains are human-adapted and rely on immune evasion/systemic spread tools such as the Vi capsule and typhoid toxin. The Vi capsule can blunt neutrophil targeting and reshape phagocyte interactions through limiting neutrophil responses while promoting macrophage uptake via DC-SIGN, while the typhoid toxin is an intracellularly produced exotoxin that causes disease [76,77]. Within non-typhoidal salmonellosis, several high-virulence serotypes frequently carry serotype-associated virulence plasmids with the spv operon, which augments intracellular survival and facilitates systemic infection [78]. Interestingly, the survival of Salmonella serotypes within the host’s macrophages varies dramatically depending on the host species. For instance, S. Typhimurium (a non-typhoidal variant) demonstrated greater survival and replication within mice compared to significant declines in viable counts of S. Typhi (typhoidal) strains within mice [79]. Similarly, S. Typhimurium induces greater macrophage death in both mouse and human cells compared to each other [79].
3.3. Evolution and Adaptation
3.3.1. Genomic Plasticity
The evolutionary success of Salmonella enterica is driven by the capacity to gain, lose, and remodel genetic material in response to host and environmental pressures [80]. Comparative genomics of Salmonella consistently supports a model in which a relatively conserved core genome is supplemented by a highly variable accessory genome concentrated in regions of genomic plasticity (RGPs), which are regions of a genome that are structurally absent in other similar genomes and are associated with frequent rearrangements facilitated by mobile genetic elements (MGEs) [80]. A large-scale analysis of 12,244 Salmonella genomes mapped genome content into regions of genome plasticity, emphasizing how strain-specific acquisition and loss events shape adaptation, pathogenicity, and antimicrobial resistance [80]. Broadly speaking, plasticity is mediated by horizontally acquired genomic islands or pathogenicity islands (PAIs), prophages (which often constitute a major fraction of accessory DNA), conjugative plasmids, and insertion sequences, which drive structural variation [81,82]. Among the best-studied drivers of Salmonella plasticity are pathogenicity islands, which are horizontally acquired loci that encode coordinated virulence functions and are frequently associated with tRNA insertion sites, integrases, and atypical GC content [83]. Although many PAIs can be lineage-specific, S. enterica broadly shares two cornerstone islands: SPI-1, which encodes effector proteins primarily involved in epithelial invasion, and SPI-2, which encodes effector proteins mainly associated with intracellular survival and replication within host cells [84]. For typhoidal serotypes, larger island-like elements such as SPI-7-related integrative conjugative elements (ICEs) and associated variation have been analyzed as mobile platforms that contribute to typhoid-specific traits and long-term adaptation [85]. Prophages are repeatedly identified as major contributors to Salmonella accessory gene content and a major mechanism for rapid diversification. Dedicated reviews emphasize that functional prophages are abundant in Salmonella genomes and can mediate lysogenic conversion, adding genes that influence fitness, stress tolerance, immune interaction, and virulence [82]. Conjugative and mobilizable plasmids are another principal engine of genomic plasticity in major Salmonella strains, particularly for antimicrobial resistance [86]. Inc-group plasmids (e.g., IncHI2) are frequently implicated in the dissemination of resistance determinants across Salmonella species [86]. For example, studies of clinical and food isolates have identified IncHI2 as a prominent plasmid lineage contributing to AMR spread in Salmonella species, with multiple MGEs and resistance modules recombining across the plasmid backbone [86].
3.3.2. Environmental Persistence and Stress Resistance
S. enterica persists outside the host across a wide range of built and natural environments, including low-moisture foods and processing facilities, farm and animal-production settings, and water/produce-associated niches, because it can rapidly adapt to desiccation, nutrient limitation, temperature shifts, oxidative and acid stress, and sanitizer exposure [87]. In “low-water-activity matrices,” Salmonella may not grow, but it can survive for extended periods, creating long-lived contamination reservoirs that are difficult to eradicate once established [87]. Salmonella persistence is amplified by surface attachment and biofilm formation on equipment and food-contact materials; biofilms protect cells from dehydration, pH extremes, and antimicrobials and are repeatedly emphasized as a central mechanism for Salmonella survival and recurring contamination in food processing environments [88]. Recent experimental data also show S. Dublin can survive and even proliferate in sterile bedding sand for days at room temperature, supporting the plausibility of persistence in sterile microenvironments [89].
Mechanistically, stress resistance in major Salmonella serotypes reflects both conserved stress-response networks and strain/serotype variation in traits that promote survival on surfaces and in harsh matrices [90]. For long-term environmental survival, extracellular matrix components (ECM components) are strongly implicated; experimental work shows these structures enhance long-term survival and desiccation resistance, making them highly relevant to persistence on dry surfaces and in low-moisture foods [90]. Regarding major Salmonella serotypes, it is most accurate to emphasize that many clinically important serotypes (such as S. Typhimurium, S. Enteritidis, S. Newport, S. Dublin, etc.) share core stress tools, while differences in persistence often arise from how strongly they form biofilms under relevant temperatures and stressors, how effectively they endure desiccation/low nutrients, and which environments they most frequently cycle through (poultry/eggs, cattle/dairy, produce/water systems), which shapes opportunities for selection and recontamination [90,91].
4. Antimicrobial Resistance (AMR) Trends
4.1. Global AMR Patterns
4.1.1. Increasing Multiple Drug-Resistant Strains
Although most Salmonella infections do not require antibiotic therapy and are managed primarily with rehydration, a significant minority of patients require antibiotics either prophylactically or for the treatment of invasive disease [92]. Prophylactic antibiotic therapy is recommended for patients at increased risk of invasive disease, including immunocompromised individuals and infants younger than three months of age [92]. Additionally, iNTS is characterized by manifestations such as bacteremia, disseminated infection, or enteric fever [92]. In these cases, prompt and effective antibiotic therapy is essential to improving outcomes, particularly among immunocompromised patients, underscoring the ongoing importance of effective antimicrobial treatments for Salmonella infections [92]. Over the past several years, there has been a marked global increase in multidrug-resistant (MDR) Salmonella strains. Reported MDR prevalence in invasive disease varies substantially across regions, ranging from 45.8% to 75% in invasive disease worldwide [93,94,95]. To improve comparability, these findings were synthesized by geographic region into a structured summary of MDR prevalence estimates, provided in Table 4.
Table 4.
Prevalence of multidrug-resistant (MDR) NTS Salmonella in clinical and food-chain isolates across regions. Confidence intervals are shown where sufficient data were available. NR = not reported; 95% confidence intervals were calculated using the normal approximation to the binomial distribution.
In Europe, a 13-year study in Italy reported MDR in 45.8% of 680 clinical isolates, while data from Romania demonstrated both a high overall prevalence of MDR isolates and a marked temporal increase from 24% to 56% between 2011 and 2021 in poultry-associated strains [96]. In Asia, analysis of 8541 clinical samples in China found that 21.9% of isolates met criteria for MDR, and 69.5% were resistant to at least one antibiotic [97]. In contrast, substantially higher MDR prevalence has been reported in sub-Saharan Africa, where rates have reached approximately 75% among NTS isolates since 2001 [95]. Notably, the high MDR prevalence reported in Romania reflects food-chain isolates from poultry products, which may not be directly comparable to clinical surveillance studies but highlights a significant upstream reservoir contributing to antimicrobial resistance. Although these estimates are derived from heterogeneous study populations and surveillance systems, the consistently high prevalence and overlapping ranges denote a substantial global burden of MDR Salmonella, with particularly elevated rates in resource-limited settings.
On the other hand, S. Typhi, a serotype primarily associated with typhoid fever in humans and increased mortality rates involving much more severe infection, has also seen large increases in incidence of AMR and MDR serotypes, while an extensively drug-resistant (XDR) strain has become dominant in Pakistan (70% in 2020) and was recently identified in Iraq [98,99]. Although XDR strain dominance has so far been limited to the Middle East, the World Health Organization (WHO), reflecting the growing public health concern, has classified both fluoroquinolone-resistant Typhoidal and NTS as “high-priority” pathogens, the second-highest tier, on its 2024 Bacterial Priority Pathogens List (BPPL), which ranks organisms based on criteria including mortality, disease burden, incidence, and resistance trends over the past decade [99,100]. Although NTS infections are typically self-limiting, this designation underscores the significant and escalating threat posed by increasing MDR Salmonella strains [100].
4.1.2. Specific Problematic Lineages
Notably, global surveillance over the past two decades indicates that several of the twenty most prevalent S. enterica serotypes have exhibited substantial increases in MDR, including S. Typhi, S. Infantis, S. I 1,4,[5],12:i:-, and S. Dublin [93,101]. Among these, the most pronounced increase in MDR prevalence has been observed in S. Typhimurium, with MDR rates reaching 73.3% [94,102]. Other serotypes with notable increases in MDR rates include S. Enteritidis (42.2%) and S. I 1,4,[5],12:i:- (36.0%), as well as S. Rissen, which has recently demonstrated resistance to as many as 13 antibiotics [93,102]. In S. Typhi, ciprofloxacin resistance has become a global issue, while ceftriaxone and fluoroquinolone resistance continue to increase along with NTS trends [98]. Alongside the rising prevalence of AMR, MDR, and XDR S. Typhi serotypes, studies have shown that only 1–4% of patients with suspected typhoid fever in endemic regions such as Asia and Africa have a culture-confirmed S. Typhi infection [103]. This low confirmation rate highlights the extensive use of empirical antibiotic therapy and the resulting selective pressure driving antimicrobial resistance in S. Typhi [97]. Beyond overall MDR prevalence, AMR trends point to the emergence and persistence of high-risk lineages within several additional serotypes, including S. Heidelberg, S. Derby, S. Muenchen, S. Thompson, and S. Senftenberg. Of particular concern, fluoroquinolone non-susceptibility has increased markedly in S. Enteritidis and S. Dublin, further limiting first-line treatment options for invasive infections [93]. Additionally, a particularly concerning MDR lineage of S. I 1,4,[5],12:i:- has been identified across Europe, Canada, Australia, and the United States, underscoring its successful international dissemination [104]. This lineage is characterized by resistance to ampicillin, streptomycin, sulfamethoxazole, and tetracycline, a resistance profile that significantly constrains therapeutic options, especially in resource-limited settings [104].
S. Infantis represents another high-risk lineage that has undergone a rapid global shift toward multidrug resistance. Once largely antibiotic-susceptible in 2014, the majority of S. Infantis isolates displayed MDR phenotypes by 2022 [105]. This transition has been driven in part by a sharp increase in extended-spectrum β-lactamase (ESBL) carriage, with prevalence estimates now approaching 60% [106]. Correspondingly, the incidence of S. Infantis infections resistant to five or more antibiotic classes increased from approximately 20% in 2010 to 80% in 2020 [106]. In Peru, iNTS surveillance revealed that 100% of S. Infantis isolates were ESBL producers, accompanied by a significant rise in the overall incidence of human disease caused by this serotype [107]. These findings align with trends observed in the United States, where Salmonella infections in 2006–2008 were dominated by S. Typhimurium and S. Heidelberg, followed by declines in these serotypes and a concurrent increase in infections attributable to S. Infantis [108].
Another emerging high-risk lineage is S. Newport REPJJP01, which was first identified as MDR in 2016 and continued to expand during the COVID-19 pandemic, despite an overall decline in Salmonella infections. By 2022, MDR prevalence in this lineage had reached 86% [109]. Importantly, this expansion has been associated with increased clinical severity, as 33% of individuals infected with S. Newport REPJJP01 required hospitalization, compared with 27% among patients infected with non-Newport NTS strains during the same period [109].
4.2. Mechanisms of Resistance
4.2.1. Plasmid-Mediated Resistance
Plasmids are extrachromosomal DNA molecules within a bacterial cell that are key mediators in horizontal gene transfer. Due to this, plasmid-mediated antimicrobial resistance plays a significant role in the emergence and dissemination of MDR Salmonella worldwide [110]. Plasmids are usually classified into incompatibility (Inc) groups, in which all members within the same group cannot be stably maintained within the same bacterial cell line over successive generations [110]. Plasmids of different Inc groups differ in their size, transfer mechanism, and even their antibiotic resistance genes [111]. Multiple plasmid incompatibility groups, including IncA/C, IncF, IncHI, and IncI1, have been strongly associated with antimicrobial resistance in Salmonella isolated from humans and animals [111].
Additionally, plasmids in Salmonella can have β-lactamase genes, including ESBLs and plasmid-mediated AmpC β-lactamases (PABL), which result in the bacterium having resistance to cephalosporins [112]. Notably, while plasmid-mediated AmpC β-lactamases such as CMY-2 were previously reported predominantly in human Salmonella isolates in South Korea, their recent detection in pigs highlights an expansion of resistance plasmids [112].
4.2.2. QRDR Mutations
Salmonella infections are often treated with fluoroquinolones or extended-spectrum beta-lactams [113]. As a result, there has been a development of plasmid-mediated quinolone resistance (PMQR), which is encoded by qnr genes [114]. These qnr genes encode pentapeptide repeat proteins, which work to give the bacterium resistance to quinolones by protecting DNA topoisomerase from the inhibitory effect of quinolones [113]. Moreover, quinolone resistance in Salmonella is primarily mediated by chromosomal point mutations within the quinolone resistance-determining regions (QRDRs) of genes encoding DNA gyrase (topoisomerase II) and DNA topoisomerase IV [109]. DNA gyrases and DNA topoisomerase IV are encoded by gyrA and gyrB genes and parC and parE genes, respectively [115]. Mutations in these QRDRs result in a lower quinolone-binding affinity of the topoisomerase enzymes, which confers resistance to these quinolone drugs [115]. Most commonly, QRDR mutations that confer resistance to quinolone drugs have been identified in a specific region of the gyrA gene, between amino acids 67 and 106 [116]. Studies have shown that gyrA QRDR mutations into codons Aspartate-87 (62%) and Serine-83 (38%) were found in 105 Salmonella strains resistant to nalidixic acid [116].
4.2.3. Carbapenem Resistance Emergence
Carbapenems are a powerful class of broad-spectrum β-lactam antibiotics that are often considered “last-line agents” or “antibiotics of last resort” due to their unique ability to withstand hydrolysis by most β-lactamases [117]. As such, carbapenems are not commonly used for treating Salmonella infections. However, there has been an emergence of carbapenem-resistant Enterobacterales (CRE) strains, including Salmonella, around the world, albeit it is still considered a rare occurrence [118]. Regardless, this emergence poses a significant public health concern due to the limited therapeutic options available for multidrug-resistant infections aside from carbapenems [119]. Furthermore, carbapenem resistance has been shown to primarily develop through the acquisition of a carbapenemase gene or the loss of porins, the latter of which results in the antibiotic not being able to be transported into the bacterium, thus rendering it nonfunctional [120]. In addition to these two mechanisms, carbapenem-resistant Salmonella strains have also been shown to have an AmpC-type β-lactamase or extended-spectrum β-lactamase [120]. As well, the recent identification of carbapenem resistance in various Salmonella strains, such as S. Mbandaka, highlights the ongoing expansion of resistance across bacterial strains, which raises concern for the future emergence of extensively drug-resistant Salmonella [121]. The major mechanisms of antimicrobial resistance in Salmonella that were discussed are summarized in Table 5.
Table 5.
Summary of the major antimicrobial resistance mechanisms in Salmonella enterica, including plasmid-mediated resistance, QRDR mutations, and carbapenem resistance.
4.3. Public Health and Clinical Implications
4.3.1. Treatment Challenges
The rising prevalence of antimicrobial resistance in Salmonella has important and interconnected consequences for both clinical care and public health systems. Alongside dramatic increases in MDR, the incidence of severe Salmonella infections has also risen, creating substantial challenges for clinical management [122]. MDR trends have disproportionately affected first-line antibiotics traditionally used to treat severe and invasive Salmonella, markedly narrowing effective treatment options, particularly in resource-poor settings where access to alternative therapies is limited [122]. At the health system level, escalating resistance contributes to longer hospital stays, increased healthcare expenditures, and higher rates of treatment failure and mortality, particularly in iNTS infections, where mortality is approximately 15%, and patient outcomes are increasingly compromised by escalating resistance and diminishing antimicrobial efficacy [95]. Regional differences in resistance trends further reflect disparities in antimicrobial stewardship infrastructure, antibiotic accessibility, and diagnostic capacity. Higher MDR prevalence in sub-Saharan Africa is often associated with widespread empiric antibiotic use and limited surveillance systems, whereas high-income regions continue to face challenges related to healthcare-associated transmission and antibiotic overuse [95,122]. Collectively, these patterns underscore that antimicrobial resistance in Salmonella represents not only a microbiological concern but also a systems-level public health challenge requiring coordinated global responses. Historically, Salmonella bacteremia—an infection requiring prompt diagnosis and rapid initiation of therapy to prevent fatal outcomes—was effectively treated with ampicillin or trimethoprim–sulfamethoxazole (TMP-SMX). However, widespread plasmid-mediated resistance has rendered both agents largely ineffective across multiple bacteremia–Salmonella strains, leading to their removal from recommended treatment regimens [123,124]. As resistance to these agents became entrenched, fluoroquinolones and third-generation cephalosporins, such as ceftriaxone, emerged as preferred therapies and were initially effective against MDR Salmonella strains beginning in the 1980s [124].
More recently, increasing resistance to fluoroquinolones and ceftriaxone has substantially eroded the utility of these critical agents. Fluoroquinolone-resistant Salmonella has become sufficiently prevalent that the WHO now classifies fluoroquinolone-resistant NTS and Typhoidal Salmonella as “high-priority” pathogens, reflecting the growing urgency of this treatment crisis [95,100,124]. Additionally, the urgent need to swiftly treat typhoidal infections has led to massive empiric antibiotic use, which, combined with low culture-confirmed S. Typhi infections, has led to a large increase in treatment failures [103]. Ceftriaxone-resistant Salmonella infections have now been documented across a wide geographic range, including the United States, multiple European countries, the Middle East, sub-Saharan Africa, South and Southeast Asia, and China, underscoring the global scale of this challenge [124]. Likewise, fluoroquinolone resistance presents a particular obstacle to effective treatment, as these agents were historically favored for their oral bioavailability, affordability, and broad accessibility, especially in low-resource settings [124]. In response to declining fluoroquinolone efficacy, azithromycin has more recently been adopted as a preferred option for serious infections. Alarmingly, resistance to azithromycin has already been reported in multiple serotypes, with one Italian study identifying near-universal resistance (99.4%), suggesting that its role as a frontline therapy for invasive Salmonella infections may be short-lived [94,124].
Surveillance data further indicate a marked rise in resistance to ceftriaxone and cefepime over the past five years, alongside increasing prevalence of strains resistant to fluoroquinolones and other third-generation cephalosporins [95]. Although carbapenems have historically been reserved as last-resort agents for severe Salmonella infections, emerging resistance to this class has now been documented in multiple strains, raising concern that even these final therapeutic options may be compromised [95]. The continued emergence and international dissemination of highly resistant Salmonella lineages therefore represent a major global public health threat, undermining effective treatment of severe Salmonella infection and disproportionately affecting vulnerable and under-resourced populations [124]. Addressing this growing crisis will require coordinated efforts, including the development of novel antimicrobial agents, expanded vaccine strategies, and rigorous enforcement of antimicrobial stewardship programs to slow the further spread of resistance [124].
4.3.2. Hospital and Community Settings
Hospital-acquired infections (HAIs) have consistently been associated with higher rates of MDR than community-acquired infections (CAIs), a pattern that also holds true for Salmonella infections [123,125]. While the overall MDR rate among CAIs is estimated at 62.5%, MDR prevalence in Salmonella infections has been reported to reach as high as 75%, underscoring the disproportionate contribution of Salmonella to the burden of antimicrobial resistance [125]. In both hospital and community contexts, antimicrobial-resistant and MDR Salmonella infections are associated with prolonged hospitalization—ranging from 0.5 to 2.2 additional days—as well as increased treatment costs when compared with infections caused by drug-susceptible strains [123].
The clinical consequences of MDR Salmonella are particularly pronounced in hospital settings. During a six-year outbreak of an MDR S. Senftenberg strain associated with HAIs, the case fatality rate reached 4.0%, markedly exceeding the global fatality rate of salmonellosis, which is typically below 1% [124]. Similarly, in Brazil, an outbreak involving ESBL-producing S. Infantis infected 140 infants in a neonatal unit, illustrating the dangerous convergence of high-level antimicrobial resistance and vulnerable, immunocompromised patient populations in healthcare-associated settings [124]. On the other hand, in the community setting, fluoroquinolone-resistant S. Typhi has emerged as the most common bacterial pathogen responsible for CAIs, reflecting the successful spread of resistant strains beyond healthcare environments [94,100]. The concurrent presence and circulation of MDR and AMR Salmonella in both hospital and community settings highlights the permeability of these environments and the potential for bidirectional transmission.
Together, the elevated prevalence and clinical impact of MDR Salmonella in both hospital and community settings reflect the global expansion of high-risk lineages, highlighting the urgent need for coordinated surveillance, infection control, and the development of novel therapeutic and preventive strategies.
4.3.3. Importance of Stewardship and Surveillance
The continued global rise in antimicrobial resistance underscores the increasing importance of antimicrobial stewardship, which emphasizes the intentional selection of appropriate, narrow-spectrum antibiotics; reduced reliance on empiric therapy when avoidable; and robust surveillance to limit the spread of resistant organisms such as S. enterica [126]. Although carbapenems are typically reserved for severe multidrug-resistant infections, the recent identification of carbapenem-resistant Salmonella illustrates that resistance can compromise even last-line treatment options [118]. These findings emphasize the need for effective surveillance systems to identify emerging resistance patterns early and guide appropriate clinical and public health responses [127]. Additionally, healthcare professionals play a critical role in antimicrobial stewardship, as they need to prescribe antimicrobials only when clearly indicated and tailor therapy based on susceptibility data [128]. Stewardship and surveillance efforts are critical to preserving antimicrobial efficacy and slowing the advance of resistant bacterial strains.
5. One Health Perspectives
The One Health approach is an interdisciplinary framework that recognizes the fundamental interdependence between human, animal, and environmental health. Many bacterial pathogens, including Salmonella, are maintained and transmitted across these interconnected systems, making it insufficient to study and control these infections solely through the lens of human disease [129]. Animal reservoirs, food production and agricultural practices, environmental contamination, and antimicrobial use collectively influence the emergence, transmission, and persistence of bacterial infections in human populations. These infections arise from complex transmission pathways involving animal reservoirs, food production systems, and environmental persistence, underscoring the need for integrated, coordinated control strategies across human, veterinary, and environmental health sectors [129].
5.1. Animal Reservoirs and Zoonotic Transmission
5.1.1. Poultry, Cattle, Swine, Reptiles, and Pets
Food-producing animals serve as the principal reservoirs for zoonotic Salmonella. Poultry, particularly chickens and turkeys, are the most significant contributors to human infection, with serotypes such as S. Enteritidis and S. Typhimurium frequently identified from both poultry flocks and human clinical cases [129]. Genetic comparisons have shown significant overlap between strains isolated from retail poultry products and those causing human disease, supporting foodborne transmission from poultry to humans [129,130]. Bacterial colonization of the avian gastrointestinal tract typically presents asymptomatically, allowing poultry birds to act as vectors for Salmonella without signs of illness, contaminating eggs, meat, and processing environments [129].
Cattle and swine also represent important reservoirs, harboring a wide diversity of Salmonella serotypes that can enter the human food supply through beef and pork products [130]. Studies of cattle herds have shown fecal shedding rates ranging from 20% to 50%, with increased shedding during transport and prior to slaughter, induced by high stress [130]. Swine production systems facilitate amplification through high-density housing and shared feed sources. Antimicrobial use in livestock has further contributed to the emergence of MDR Salmonella strains, including those resistant to fluoroquinolones and third-generation cephalosporins, which are commonly used to treat invasive infections in humans [131,132].
Non-food animals also contribute to zoonotic transmission, with an emphasis on young children who have these animals as household pets. Reptiles such as turtles, snakes, and lizards frequently carry Salmonella as part of their normal intestinal flora. Reptile-associated Salmonella strains account for approximately 6% of sporadic Salmonella infections in the United States, disproportionately affecting young children [133]. Common indoor pets, including dogs and cats, may become infected through contaminated pet food or raw meat diets and can transmit Salmonella to humans within households [26]. This inter-species transmission highlights the fact that Salmonella transmission through animals is not solely limited to food production settings but also occurs in domestic environments.
5.1.2. Food Production Chain Dynamics
Although animals serve as the primary source of Salmonella, transmission is amplified throughout the food production chain. Contamination may occur at many points during the food production process, including during animal rearing, slaughter, processing, or distribution. Once introduced into processing facilities, Salmonella can persist by forming biofilms on equipment and surfaces, protecting the bacteria from disinfectants, allowing for long-term survival and widespread contamination [134]. Additionally, modern centralized food processing systems have increased the risk of widespread outbreaks. The large quantities of food are produced centrally and distributed over the globalized supply chains, encompassing wide geographic areas. A single contaminated product can therefore lead to infections across multiple states. Fresh produce, once considered a low-risk vehicle, has increasingly been implicated in outbreaks due to contamination from animal manure, irrigation water, or wildlife intrusion [134]. Surveillance data indicate that fruits and vegetables accounted for nearly 46% of foodborne illnesses in the United States between 1998 and 2013 [135]. These dynamics emphasize that Salmonella control must address agricultural and environmental sources at every stage from production to fork rather than relying solely on food preparation practices.
5.2. Environmental Persistence
5.2.1. Water Systems
Environmental reservoirs play an important role in maintaining Salmonella outside animal hosts. Surface waters such as rivers, lakes, and irrigation canals can become contaminated through agricultural runoff, wastewater discharge, and wildlife fecal matter. Salmonella is capable of surviving for extended periods in aquatic environments, particularly within sediments and biofilms that protect the organism from environmental stress, facilitating repeated contamination of crops and recreational waters [136]. Moreover, waterborne transmission has been increasingly recognized in produce-associated outbreaks. Investigations have identified contaminated irrigation water as a direct source of Salmonella on leafy greens and other vegetables consumed without cooking [137]. Climate-related factors, including flooding and heavy rainfall, further increase this risk by spreading fecal contamination and overwhelming water treatment systems, redistributing pathogens across agricultural landscapes [138].
5.2.2. Agricultural Runoff
Agricultural runoff is a major pathway by which animal-associated Salmonella enters soil and water environments. The use of untreated or inadequately treated animal manure as fertilizer introduces viable bacteria into soil, where Salmonella may survive for months depending on temperature and moisture [139]. Runoff from concentrated animal feeding operations (CAFOs) can transport the organism into nearby waterways used for irrigation or recreation, concentrating downstream water sources and crops. These pathways are particularly concerning in regions where livestock density overlaps with produce farming, creating opportunities for cross-sectoral pathogen transfer. The persistence of antimicrobial-resistant Salmonella in agricultural environments further compounds the challenge, as resistance genes can be maintained and disseminated through environmental microbial communities and transferred to other bacteria, reinforcing connections between antimicrobial use and resistance patterns in human infection [138,139,140].
5.2.3. Wildlife Reservoirs
Wildlife species, including birds, rodents, and wild mammals, contribute to the environmental maintenance of Salmonella. These animals can acquire infection from contaminated environments and disseminate the pathogen through fecal shedding across farms and natural habitats. Migratory birds, in particular, have been implicated in the long-distance spread of certain Salmonella serotypes, linking geographically distant ecosystems to one another [141]. Wildlife intrusion into agricultural fields has been associated with produce contamination, reinforcing the need for ecological considerations within food safety frameworks.
5.3. Integrated Control Efforts
5.3.1. Cross-Sectoral Surveillance and Communication
Effective control of Salmonella requires coordinated multiple-sector surveillance across human health, veterinary, and environmental sectors. Integrated systems such as the U.S. National Antimicrobial Resistance Monitoring System (NARMS) monitor Salmonella isolates across clinical infections, retail meats, and food animals, providing critical insights into transmission patterns and resistance trends [132]. WGS has further enhanced outbreak detection and source attribution by allowing precise strain comparison and timely public health interventions. These surveillance efforts are most effective when paired with inter-sectional communication. Rapid data sharing between public health agencies, agricultural producers, and environmental regulators facilitates early outbreak identification and coordinated responses that target upstream sources of contamination rather than focusing only on clinical cases [132].
5.3.2. Lessons from Recent Outbreaks Tied to Agriculture and Environment
Recent Salmonella outbreaks illustrate the importance of One Health Approaches. Limitations of isolated treatment approaches that focus on only one part of the transmission pathway are not sufficient for effective, widespread pathogen eradication. Supporting this, a One Health European surveillance mapping study of the Salmonella pork meat chain in France demonstrated how transmission and surveillance operate across the farm-to-fork continuum, spanning three interconnected sectors: animal health (farm and transport), food safety (slaughterhouse, processing plant, and retail), and public health (general population) [133]. This work highlighted that, despite the presence of surveillance activities within each sector, fragmentation in data flow, limited harmonization of laboratory methods and case definitions, and gaps in inter-sector communication can delay detection and hinder coordinated response efforts [26]. Multistate outbreaks linked to poultry, beef, and fresh produce have repeatedly demonstrated how failures in animal management, water quality, or environmental controls can precipitate widespread human disease [142,143,144]. Furthermore, analyses of outbreak-associated serotypes demonstrate overlap with strains circulating in food animals and agricultural environments. Preventive strategies such as poultry vaccination, improved manure treatment, water irrigation monitoring, and antimicrobial stewardship have been shown to reduce Salmonella prevalence at multiple points along the transmission pathway. Interventions targeting a single sector are insufficient; instead, sustained reductions in Salmonella burden require simultaneous improvements in animal husbandry, environmental management, food processing hygiene, and consumer education. By addressing shared risk factors across human, animal, and environmental systems, the One Health framework provides a comprehensive approach for reducing the burden of Salmonella infections while supporting food safety and public health [144].
6. Prevention & Control of Salmonella
Salmonella causes disease through two closely related but epidemiologically distinct pathways, and effective prevention depends on recognizing these differences. NTS is most often associated with animal reservoirs and the food production chain, with transmission occurring through contaminated foods, cross-contamination during preparation, and direct animal contact in certain settings [145]. In contrast, typhoidal Salmonella is primarily maintained through human reservoirs and spreads via the fecal–oral route, particularly in areas where water quality, sanitation, and hygiene practices are inadequate. Prolonged shedding and chronic carriage can further sustain transmission [146]. Table 6 synthesizes these concepts by contrasting non-typhoidal and typhoidal Salmonella across key domains, including reservoir, transmission routes, and the highest-yield prevention strategies, providing a practical framework for translating epidemiology into targeted control measures.
Table 6.
Key differences in reservoirs, transmission pathways, and prevention strategies for non-typhoidal versus typhoidal Salmonella (NTS vs. S. Typhi/S. Paratyphi).
Novel approaches to disease prevention for NTS increasingly rely on advanced biotechnology, including the development of various human vaccine candidates and the integration of genomics technology into public health surveillance. Innovative vaccine platforms are currently in the pipeline, such as iNTS-GMMA, which utilizes outer membrane vesicles to elicit a broad bactericidal antibody response, and glycoconjugate subunits like OSP-rT2544 that offer potential cross-protection against multiple Salmonella serovars [33]. Furthermore, research into reverse vaccinology and subunit vaccines targeting conserved proteins like InvH is showing promise in animal models. In tandem with these medical advancements, the use of WGS within surveillance networks like PulseNet has revolutionized outbreak management by allowing for the rapid identification of related bacterial clusters and the precise tracing of contamination sources [33]. However, implementing these sophisticated measures in low- and middle-income countries (LMICs), particularly in high-burden regions like sub-Saharan Africa, presents formidable challenges. These hurdles include high production costs, limited coverage across diverse regional strains, and the logistical difficulty of integrating new vaccines into existing national immunization programs [33]. To enhance the value of public health policy, global strategies must address these barriers while tailoring interventions to local agricultural practices and regulatory frameworks, as traditional food safety measures alone are often insufficient to achieve sustained control in these high-risk environments.
In summary, prevention strategies for Salmonella should be aligned with the organism’s reservoir and dominant route of spread. Reducing NTS burden relies on integrated food safety measures across production, processing, and consumer handling, supported by hygiene practices and targeted protections for vulnerable populations [145,146]. Limiting typhoidal Salmonella transmission requires improvements in water and sanitation systems, consistent hand hygiene, timely diagnosis and appropriate antimicrobial therapy, and vaccination in endemic areas, among travelers, and during outbreaks when indicated [147,149]. Across both entities, robust surveillance and coordinated outbreak response remain essential to identify sources, implement control measures efficiently, and monitor antimicrobial resistance trends.
7. Gaps in Knowledge and Future Research Needs
7.1. Global WGS Integration Challenges
Since its inception, WGS has become the gold standard for characterizing microbial genomes and linking genetic variation to clinically and epidemiologically relevant phenotypes [169,170,171]. Over the past two decades, declining costs have eliminated major financial barriers, shifting the primary challenges of global WGS integration from technology to international participation and coordination [171,172,173].
Many countries remain hesitant to engage in global surveillance platforms such as Pathogenwatch, NCBI Pathogen Detection, and GenomeTrakr due to data protection laws, regulatory constraints, and concerns over data ownership and privacy [173,174,175]. This fragmentation limits effective global Salmonella surveillance. As WGS becomes standard, cross-country comparability is essential; however, harmonization of typing methods remains inadequate, particularly core genome multilocus sequence typing (cgMLST) and whole genome multilocus sequence typing (wgMLST) [169,173,175,176,177,178]. Additionally, an effective data sharing capability may depend on a decentralized database where improved visualization tools are needed to integrate phylogenetic, geographic, and temporal data at both global and local scales [173,174,175].
7.2. Understudied Serotypes
Many non-dominant Salmonella serotypes remain poorly characterized despite their potential clinical and public health importance. While surveillance focuses on dominant serotypes such as S. Typhimurium, S. Newport, and S. Enteritidis, understudied serotypes, such as S. Rubislaw, S. Schwarzengrund, S. Braenderup, S. Saintpaul, S. Muenchen, S. Montevideo, and S. Weltevreden, exhibit distinct epidemiological and genomic features [179,180,181,182,183,184,185,186]. Also, multiple serotypes were observed coexisting within single environmental water sources, highlighting ecological complexity [179,185,187,188]. The BEAM (Bacteria, Enterics, Amoeba, and Mycotics) Dashboard (Table 7) demonstrates the top 10 most common NTS serotypes over the last two years, with S. Enteritidis and S. Newport being among the most frequent ones, while four of the listed serotypes are understudied [23,189].
Table 7.
CDC’s Bacteria, Enterics, Amoeba, and Mycotics Dashboard of the top 10 Salmonella serotypes (2024–2025) in descending order by total number of isolates as of 27 February 2026 [189].
Environmental factors, particularly seasonal rainfall and hydrology, were stronger predictors of Salmonella presence and diversity than land use or proximity to agriculture, challenging assumptions about farm-dominated sources [185,187]. Genomic analyses revealed notable serotype-specific traits, including the first report of SPI-10 in S. Braenderup, SGI-1 in poultry-associated S. Schwarzengrund, and CS54 islands limited to S. Saintpaul and S. Braenderup [190,191], with S. Saintpaul demonstrating low plasmid diversity [190,192]. Moreover, the discovery of previously uncharacterized genetic elements, such as aerobactin biosynthesis genes linked to avian adaptation, underscores major gaps in understanding serotype-specific pathogenicity [190,191]. These findings suggest that understudied serotypes may have unrecognized epidemiological and clinical significance.
7.3. AMR Surveillance Gaps
Across multiple studies, AMR in Salmonella shows strong but imperfect associations with serotype, sequence type (ST), and source [193,194,195,196,197]. Common serotypes such as S. Typhimurium, S. Enteritidis, S. Weltevreden, S. Typhi, and S. Rissen frequently exhibit ST-specific lineages, with ST34 emerging as an evolutionarily successful backbone capable of accommodating diverse serotype determinants [195,196,197,198,199]. However, repeated identification of unexpected serotype–ST combinations suggests frequent horizontal gene transfer, decoupling serotype from resistance and virulence profiles [195]. This is particularly concerning for S. Typhimurium, which carries the largest documented AMR burden and may serve as a key reservoir for transmissible resistance genes, the full extent of whose spread remains poorly understood, especially under selective pressures such as serotype-specific vaccination [94,191,195,196,197,198,199].
Resistance patterns vary substantially by antimicrobial class, host source, and time [197,198,200]. Tetracycline resistance was consistently high across studies, peaking at 77.3% in some datasets, with sulfonamide and streptomycin resistance also commonly reported [190,192,195,197,199,201,202]. Ampicillin resistance generally increased over time but showed regional declines in more recent years [94,195,198]. Fluoroquinolone resistance, including ciprofloxacin, doubled by 2020 before declining in 2022; however, multiple animal-associated studies report substantial ciprofloxacin and azithromycin resistance that is not consistently captured in routine surveillance systems [94,195,198]. Resistance to historical first-line drugs such as chloramphenicol and cephalosporins remains rare in some clinical datasets; it is markedly higher in poultry and livestock isolates [195,198].
Source attribution is another major factor associated with AMR surveillance gaps. More than 50% of resistant isolates originated from food and animal feed sources, with AMR prevalence often exceeding that observed in human clinical isolates [38,190,191,197]. Resistance genes such as sul1, tetA, and tetR were frequently detected even in production settings where antimicrobials were reportedly not administered, suggesting environmental persistence and indirect selection pressures. Emerging MDR lineages, including a novel S. Montevideo cluster (ST-10844) with approximately 80% MDR prevalence in China, underscore the growing threat posed by understudied serotypes that fall outside dominant surveillance targets [35,94,197].
8. Conclusions and Future Directions
Salmonella remains a pervasive global public health threat, characterized by a massive burden of illness and significant mortality across both typhoidal and non-typhoidal serotypes. The pathogen’s remarkable ability to adapt through genomic plasticity and persist in diverse environmental reservoirs underscores the necessity of a One Health approach, which integrates human, veterinary, and environmental health sectors to disrupt complex transmission pathways.
While technological advancements such as WGS have revolutionized outbreak detection and source attribution, significant challenges remain regarding international data-sharing integration and the characterization of understudied serotypes. Furthermore, the escalating prevalence of MDR and XDR strains severely limits traditional treatment options, making robust antimicrobial stewardship and the development of novel therapeutic or vaccine strategies urgent priorities. Ultimately, sustained reductions in the global Salmonella burden will require continued cross-sectoral collaboration, enhanced surveillance harmonization, and a deeper understanding of the ecological and molecular drivers of this resilient pathogen.
Author Contributions
A.R. led the writing of this review article along with significant contributions from M.C., N.J.S., J.K., B.D., M.K., N.M., B.T., A.H. and P.K. Additionally, T.S.D. provided valuable guidance throughout the writing process and was responsible for the critical editing of this manuscript. All authors have read and agreed to the published version of the manuscript.
Funding
This research received no external funding.
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
The original contributions presented in this study are included in the article. Further inquiries can be directed to the corresponding author.
Acknowledgments
The authors gratefully acknowledge the University of Central Florida College of Medicine FIRE+ Program for providing the opportunity and supportive environment that facilitated this collaborative scholarly work.
Conflicts of Interest
The authors declare no conflict of interest.
References
- Holt, J.G.; Krieg, N.R.; Sneath, P.H.A.; Staley, J.T.; Williams, S.T. Bergey’s Manual of Determinative Bacteriology, 9th ed.; Williams & Wilkins: Baltimore, MD, USA, 1994. [Google Scholar]
- Tindall, B.J.; Grimont, P.A.D.; Garrity, G.M.; Euzéby, J.P. Nomenclature and taxonomy of the genus Salmonella. Int. J. Syst. Evol. Microbiol. 2005, 55, 521–524. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Brenner, F.W.; Villar, R.G.; Angulo, F.J.; Tauxe, R.; Swaminathan, B. Salmonella nomenclature. J. Clin. Microbiol. 2000, 38, 2465–2467. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Porwollik, S.; Boyd, E.F.; Choy, C.; Cheng, P.; Florea, L.; Proctor, E.; McClelland, M. Characterization of Salmonella enterica subspecies I genovars by use of microarrays. J. Bacteriol. 2004, 186, 5883–5898. [Google Scholar] [CrossRef] [Scilit]
- Gal-Mor, O. Persistent Infection and Long-Term Carriage of Typhoidal and Nontyphoidal Salmonellae. Clin. Microbiol. Rev. 2018, 32, e00088-18. [Google Scholar] [CrossRef] [Scilit]
- Dougan, G.; Baker, S. Salmonella enterica serovar Typhi and the pathogenesis of typhoid fever. Annu. Rev. Microbiol. 2014, 68, 317–336. [Google Scholar] [CrossRef] [Scilit]
- Haselbeck, A.H.; Panzner, U.; Im, J.; Baker, S.; Meyer, C.G.; Marks, F. Current perspectives on invasive nontyphoidal Salmonella disease. Curr. Opin. Infect. Dis. 2017, 30, 498–503. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Uche, I.V.; MacLennan, C.A.; Saul, A. A Systematic Review of the Incidence, Risk Factors and Case Fatality Rates of Invasive Nontyphoidal Salmonella (iNTS) Disease in Africa (1966 to 2014). PLoS Neglected Trop. Dis. 2017, 11, e0005118. [Google Scholar] [CrossRef] [Scilit]
- Hanning, I.B.; Nutt, J.D.; Ricke, S.C. Salmonellosis outbreaks in the United States due to fresh produce: Sources and potential intervention measures. Foodborne Pathog. Dis. 2009, 6, 635–648. [Google Scholar] [CrossRef] [Scilit]
- Lamichhane, B.; Mawad, A.M.M.; Saleh, M.; Kelley, W.G.; Harrington, P.J., 2nd; Lovestad, C.W.; Amezcua, J.; Sarhan, M.M.; El Zowalaty, M.E.; Ramadan, H.; et al. Salmonellosis: An Overview of Epidemiology, Pathogenesis, and Innovative Approaches to Mitigate the Antimicrobial Resistant Infections. Antibiotics 2024, 13, 76. [Google Scholar] [CrossRef] [Scilit]
- He, Y.; Jia, Q.; Cai, K.; Xu, S.; Li, H.; Xie, Q.; Qiu, Y.; Zhang, L.; Jiao, X. The global, regional, and national burden of Invasive Non-typhoidal Salmonella (iNTS): An analysis from the Global Burden of Disease Study 1990–2021. PLoS Neglected Trop. Dis. 2025, 19, e0012960. [Google Scholar] [CrossRef] [Scilit]
- Ghunaim, H.; Desin, T.S. Potential Impact of Food Safety Vaccines on Health Care Costs. Foodborne Pathog. Dis. 2015, 12, 733–740. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kumar, G.; Kumar, S.; Jangid, H.; Dutta, J.; Shidiki, A. The rise of non-typhoidal Salmonella: An emerging global public health concern. Front. Microbiol. 2025, 16, 1524287. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Marshall, K.E.; Nguyen, T.; Ablan, M.; Nichols, M.C.; Robyn, M.P.; Sundararaman, P.; Whitlock, L.; Wise, M.E.; Jhung, M.A. Investigations of possible multistate outbreaks of Salmonella, Shiga toxin–producing Escherichia coli, and Listeria monocytogenes infections—United States, 2016. MMWR Surveill. Summ. 2020, 69, 1–14. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Majowicz, S.E.; Musto, J.; Scallan, E.; Angulo, F.J.; Kirk, M.; O’Brien, S.J.; Jones, T.F.; Fazil, A.; Hoekstra, R.M. The global burden of nontyphoidal Salmonella gastroenteritis. Clin. Infect. Dis. 2010, 50, 882–889. [Google Scholar] [CrossRef] [Scilit]
- U.S. Department of Agriculture Food Safety and Inspection Service. Salmonella By The Numbers. Available online: https://www.fsis.usda.gov/inspection/inspection-programs/inspection-poultry-products/reducing-salmonella-poultry/salmonella (accessed on 30 March 2026).
- European Food Safety Authority. The European Union One Health 2024 zoonoses report. EFSA J. 2025, 23, e9759. [Google Scholar] [CrossRef] [Scilit]
- Scallan Walter, E.J.; Cui, Z.; Tierney, R.; Griffin, P.M.; Hoekstra, R.M.; Payne, D.C.; Rose, E.B.; Devine, C.; Namwase, A.S.; Mirza, S.A.; et al. Foodborne illness acquired in the United States—Major pathogens, 2019. Emerg. Infect. Dis. 2025, 31, 669–677. [Google Scholar] [CrossRef] [Scilit]
- Ayuti, S.R.; Khairullah, A.R.; Al-Arif, M.A.; Lamid, M.; Warsito, S.H.; Moses, I.B.; Hermawan, I.P.; Silaen, O.S.M.; Lokapirnasari, W.P.; Aryaloka, S.; et al. Tackling salmonellosis: A comprehensive exploration of risk factors, impacts, and solutions. Open Vet. J. 2024, 14, 1313–1329. [Google Scholar] [CrossRef] [Scilit]
- Diemert, S.; Yan, T. Clinically unreported salmonellosis outbreak detected via comparative genomic analysis of municipal wastewater Salmonella isolates. Appl. Environ. Microbiol. 2019, 85, e00139-19. [Google Scholar] [CrossRef] [Scilit]
- Weller, D.L.; Tierney, R.; Verlander, S.; Bruce, B.B.; Rose, E.B. Disparities in Salmonellosis Incidence for US Counties with Different Social Determinants of Health Profiles Are Also Mediated by Extreme Weather: A Counterfactual Analysis of Laboratory Enteric Disease Surveillance (LEDS) Data From 1997 through 2019. J. Food Prot. 2024, 87, 100379. [Google Scholar] [CrossRef] [Scilit]
- Gilchrist, J.J.; MacLennan, C.A.; Hill, A.V.S. Genetic susceptibility to invasive Salmonella disease. Nat. Rev. Immunol. 2015, 15, 452–463. [Google Scholar] [CrossRef] [Scilit]
- Global Burden of Disease Study 2017 Collaborators. The global burden of non-typhoidal Salmonella invasive disease: A systematic analysis for the Global Burden of Disease Study 2017. Lancet Infect. Dis. 2019, 19, 1312–1324. [Google Scholar] [CrossRef] [Scilit]
- Cox, J.M.; Pavic, A. Salmonella: Introduction. In Encyclopedia of Food Microbiology, 2nd ed.; Batt, C.A., Tortorello, M.L., Eds.; Academic Press: Cambridge, MA, USA, 2014; pp. 322–331. [Google Scholar]
- Teklemariam, A.D.; Al-Hindi, R.R.; Albiheyri, R.S.; Alharbi, M.G.; Alghamdi, M.A.; Filimban, A.A.R.; Al Mutiri, A.S.; Al-Alyani, A.M.; Alseghayer, M.S.; Almaneea, A.M.; et al. Human salmonellosis: A continuous global threat in the farm-to-fork food safety continuum. Foods 2023, 12, 1756. [Google Scholar] [CrossRef] [Scilit]
- Galán-Relaño, Á.; Valero Díaz, A.; Huerta Lorenzo, B.; Gómez-Gascón, L.; Mena Rodríguez, M.Á.; Carrasco Jiménez, E.; Pérez Rodríguez, F.; Astorga Márquez, R.J. Salmonella and salmonellosis: An update on public health implications and control strategies. Animals 2023, 13, 3666. [Google Scholar] [CrossRef] [Scilit]
- Pulford, C.V.; Perez-Sepulveda, B.M.; Canals, R.; Bevington, J.A.; Bengtsson, R.J.; Wenner, N.; Rodwell, E.V.; Kumwenda, B.; Zhu, X.; Bennett, R.J.; et al. Stepwise evolution of Salmonella Typhimurium ST313 causing bloodstream infection in Africa. Nat. Microbiol. 2021, 6, 327–338. [Google Scholar] [CrossRef] [Scilit]
- Napoleoni, M.; Villa, L.; Barco, L.; Lucarelli, C.; Tiengo, A.; Baggio, G.; Dionisi, A.M.; Angellotti, A.; Ferretti, E.; Ruggeri, S.; et al. Monophasic variant of Salmonella Typhimurium 4,[5],12:i:- outbreak in central Italy linked to porchetta consumption. Microorganisms 2023, 11, 2567. [Google Scholar] [CrossRef] [Scilit]
- Kim, M.B.; Lee, Y.J. Emergence of Salmonella Infantis carrying a pESI-like plasmid from eggs in egg grading and packing plants in Korea. Food Microbiol. 2024, 122, 104568. [Google Scholar] [CrossRef] [Scilit]
- Alvarez, D.M.; Barrón-Montenegro, R.; Conejeros, J.; Rivera, D.; Undurraga, E.A.; Moreno-Switt, A.I. A review of the global emergence of multidrug-resistant Salmonella enterica serovar Infantis. Int. J. Food Microbiol. 2023, 403, 110297. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Piña-Iturbe, A.; Tichy-Navarro, D.; Miranda-Riveros, J.; Navarrete, M.J.; Moreno-Switt, A.I. Emergent Salmonella enterica serovar Infantis forms a monophyletic lineage shaped by geographic structuring. Int. J. Food Microbiol. 2026, 446, 111536. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Centers for Disease Control and Prevention. Foodborne Illness Source Attribution Estimates—United States, 2022; Centers for Disease Control and Prevention: Atlanta, GA, USA, 2024. Available online: https://www.cdc.gov/ifsac/php/data-research/annual-report-2022.html (accessed on 27 February 2026).
- Ranjan, A.; Patel, A.; Wolfram, A.; Lakshmi, S.; Desin, T.S. Non-typhoidal Salmonella: Decoding mechanisms for effective disease control. In Salmonella—Molecular Biology, Pathogenesis, and Public Health Impact; IntechOpen: London, UK, 2025. [Google Scholar] [CrossRef] [Scilit]
- Centers for Disease Control and Prevention. Reports of Selected Salmonella Outbreak Investigations; Centers for Disease Control and Prevention: Atlanta, GA, USA, 2025. Available online: https://www.cdc.gov/salmonella/outbreaks/index.html (accessed on 30 March 2026).
- Centers for Disease Control and Prevention. How Salmonella Infections Happen. 2024. Available online: https://www.cdc.gov/salmonella/spread/index.html (accessed on 27 February 2026).
- Centers for Disease Control and Prevention. Enteric Disease Outbreaks Associated with Animal Contact—Animal Contact Outbreak Surveillance System, United States, 2009–2021. 2025. Available online: https://www.cdc.gov/mmwr/volumes/74/ss/ss7403a1.htm (accessed on 27 February 2026).
- World Health Organization. Data Collection Toolboxes. 2025. Available online: https://www.who.int/emergencies/outbreak-toolkit/investigating-outbreak-of-unknown-disease (accessed on 27 February 2026).
- Centers for Disease Control and Prevention. Multistate Foodborne Outbreaks: Investigation Steps. 2025. Available online: https://www.cdc.gov/foodborne-outbreaks/outbreak-basics/investigation-steps.html (accessed on 27 February 2026).
- Reintjes, R.; Zanuzdana, A. Outbreak investigations. In Modern Infectious Disease Epidemiology; Krämer, A., Kretzschmar, M., Krickeberg, K., Eds.; Springer: Berlin/Heidelberg, Germany, 2009; pp. 147–162. [Google Scholar] [CrossRef] [Scilit]
- Spina, A.; Rossetto, E.V.; Batra, N. Field epidemiology and outbreak investigation. In Infectious Disease Emergencies: Preparedness and Response; Fisher, D., Ed.; NUS Press: Singapore, 2025; Available online: https://emergencies.pubpub.org/pub/field-epidemiology (accessed on 27 February 2026).
- Fefferman, N.H.; Blum, M.J.; Bourouiba, L.; Gibson, N.L.; He, Q.; Miller, D.L.; Papeș, M.; Pasquale, D.K.; Verheyen, C.; Ryan, S.J. Identifying outbreak risk factors through case-control comparisons. Commun. Med. 2025, 5, 210. [Google Scholar] [CrossRef] [Scilit]
- World Health Organization. Communicable Disease Surveillance and Response Systems: Guide to Monitoring and Evaluating; World Health Organization: Geneva, Switzerland, 2006. [Google Scholar]
- Li, H.; Wu, Y.; Feng, D.; Jiang, Q.; Li, S.; Rong, J.; Zhong, L.; Methner, U.; Baxter, L.; Ott, S.; et al. Centralized industrialization of pork in Europe and America contributes to the global spread of Salmonella enterica. Nat. Food 2024, 5, 413–422. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gould, L.H.; Kline, J.; Monahan, C.; Vierk, K. Outbreaks of disease associated with food imported into the United States, 1996–2014. Emerg. Infect. Dis. 2017, 23, 525–528. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, Z.; Zhou, H.; Liu, Y.; Huang, C.; Chen, J.; Siddique, A.; Yin, R.; Jia, C.; Li, Y.; Zhao, G.; et al. Nationwide trends and features of human salmonellosis outbreaks in China. Emerg. Microbes Infect. 2024, 13, 2372364. [Google Scholar] [CrossRef] [Scilit]
- Centers for Disease Control and Prevention. Salmonella Infections Linked to Cavi Brand Whole, Fresh Papayas (June 2019). 2024. Available online: https://archive.cdc.gov/www_cdc_gov/salmonella/uganda-06-19/index.html (accessed on 27 February 2026).
- Ford, L.; Shah, H.J.; Eikmeier, D.; Hanna, S.; Chen, J.; Tagg, K.A.; Langley, G.; Payne, D.C.; Plumb, I.D. Antimicrobial-resistant nontyphoidal Salmonella infection following international travel—United States, 2018–2019. J. Infect. Dis. 2023, 228, 533–541. [Google Scholar] [CrossRef] [Scilit]
- Habrun, C.A.; Birhane, M.G.; François, L.K.; Benedict, K.; Bottichio, L.; Nemechek, K.; Tolar, B.; Schroeder, M.N.; Chen, J.C.; Caidi, H.; et al. Multistate nontyphoidal Salmonella and Shiga toxin–producing Escherichia coli outbreaks linked to international travel—United States, 2017–2020. Epidemiol. Infect. 2024, 152, e17. [Google Scholar] [CrossRef] [Scilit]
- Anagnostopoulos, L.; Vasileiadis, S.; Kourentis, L.; Voulgaridi, I.; Mouchtouri, V.A. Acute gastroenteritis in large passenger vessels. Popul. Med. 2025, 7, A15. [Google Scholar]
- Mileto, I.; Romano, G.; Gaiarsa, S.; Grassia, G.; Bagnarino, J.; Piralla, A.; Monzillo, V.; Cambieri, P.; Baldanti, F.; Corbella, M. Whole-genome sequencing as a reliable alternative for Salmonella serotyping: A comparative study with the gold-standard method. Front. Microbiol. 2025, 16, 1685741. [Google Scholar] [CrossRef] [Scilit]
- Rose, E.B.; Steele, M.K.; Tolar, B.; Pettengill, J.; Batz, M.; Bazaco, M.; Tameru, B.; Cui, Z.; Lindsey, R.L.; Simmons, M.; et al. Attribution of Salmonella enterica to food sources using whole-genome sequencing data. Emerg. Infect. Dis. 2025, 31, 783–790. [Google Scholar] [CrossRef] [Scilit]
- McDermott, P.F.; Tyson, G.H.; Kabera, C.; Chen, Y.; Li, C.; Folster, J.P.; Ayers, S.L.; Lam, C.; Tate, H.P.; Zhao, S. Whole-genome sequencing for detecting antimicrobial resistance in nontyphoidal Salmonella. Antimicrob. Agents Chemother. 2016, 60, 5515–5520. [Google Scholar] [CrossRef] [Scilit]
- Davedow, T.; Carleton, H.; Kubota, K.; Palm, D.; Schroeder, M.; Gerner-Smidt, P.; Al-Jardani, A.; Chinen, I.; Kam, K.M.; Smith, A.M.; et al. PulseNet International survey on the implementation of whole-genome sequencing in low- and middle-income countries for foodborne disease surveillance. Foodborne Pathog. Dis. 2022, 19, 332–340. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Parcell, B.J.; Gillespie, S.H.; Pettigrew, K.A.; Holden, M.T.G. Clinical perspectives in integrating whole-genome sequencing into the investigation of healthcare and public health outbreaks—Hype or help? J. Hosp. Infect. 2021, 109, 1–9. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kubota, K.A.; Wolfgang, W.J.; Baker, D.J.; Boxrud, D.; Turner, L.; Trees, E.; Carleton, H.A.; Gerner-Smidt, P. PulseNet and the changing paradigm of laboratory-based surveillance for foodborne diseases. Public Health Rep. 2019, 134, 22S–28S. [Google Scholar] [CrossRef] [Scilit]
- Timme, R.E.; Rand, H.; Sanchez Leon, M.; Hoffmann, M.; Strain, E.; Allard, M.; Roberson, D.; Baugher, J.D. GenomeTrakr proficiency testing for foodborne pathogen surveillance: An exercise from 2015. Microb. Genom. 2018, 4, e000185. [Google Scholar] [CrossRef] [Scilit]
- Sarno, E.; Pezzutto, D.; Rossi, M.; Liebana, E.; Rizzi, V. A review of significant European foodborne outbreaks in the last decade. J. Food Prot. 2021, 84, 2059–2070. [Google Scholar] [CrossRef] [Scilit]
- Savelli, C.J.; Bradshaw, A.; Ben Embarek, P.; Mateus, C. The FAO/WHO International Food Safety Authorities Network in review, 2004–2018. Foodborne Pathog. Dis. 2019, 16, 480–488. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pico-Rodríguez, J.T.; Martínez-Jarquín, H.; Gómez-Chávez, J.J.; Juárez-Ramírez, M.; Martínez-Chavarría, L.C. Effect of Salmonella pathogenicity island 1 and 2 deletion on intestinal colonization and systemic dissemination in chickens. Vet. Res. Commun. 2024, 48, 49–60. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dos Santos, A.M.P.; Ferrari, R.G.; Conte-Junior, C.A. Virulence factors in Salmonella Typhimurium: The sagacity of a bacterium. Curr. Microbiol. 2019, 76, 762–773. [Google Scholar] [CrossRef] [Scilit]
- Mishra, C.; Sahoo, S.K.; Misra, N.; Kushwaha, G.S.; Suar, M. Recent progress in molecular mechanisms of Salmonella effectors involved in gut epithelium invasion. Mol. Biol. Rep. 2025, 52, 601. [Google Scholar] [CrossRef] [Scilit]
- Tambassi, M.; Berni, M.; Bracchi, C.; Menozzi, I.; Dodi, A.; Mazzera, L.; Morganti, M.; Scaltriti, E.; Pongolini, S. Salmonella pathogenicity island 1 undergoes decay in serotypes adapted to swine and poultry. Microbiol. Spectr. 2025, 13, e0264324. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Alghoribi, M.F.; Doumith, M.; Alrodayyan, M.; Al Zayer, M.; Köster, W.L.; Muhanna, A.; Aljohani, S.M.; Balkhy, H.H.; Desin, T.S.S. Enteritidis and S. Typhimurium Harboring SPI-1 and SPI-2 Are the Predominant Serotypes Associated With Human Salmonellosis in Saudi Arabia. Front. Cell. Infect. Microbiol. 2019, 9, 187. [Google Scholar] [CrossRef] [Scilit]
- Hu, Q.; Coburn, B.; Deng, W.; Li, Y.; Shi, X.; Lan, Q.; Wang, B.; Coombes, B.K.; Finlay, B.B. Salmonella enterica serovar Senftenberg human clinical isolates lacking SPI-1. J. Clin. Microbio. 2008, 46, 1330–1336. [Google Scholar] [CrossRef] [Scilit]
- Rehman, T.; Yin, L.; Latif, M.B.; Chen, J.; Wang, K.; Geng, Y.; Huang, X.; Abaidullah, M.; Guo, H.; Ouyang, P. Adhesive mechanism of different Salmonella fimbrial adhesins. Microb. Pathog. 2019, 137, 103748. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lu, J.; Wu, H.; Wu, S.; Wang, S.; Fan, H.; Ruan, H.; Qiao, J.; Caiyin, Q.; Wen, M. Salmonella: Infection mechanism and control strategies. Microbiol. Res. 2025, 292, 128013. [Google Scholar] [CrossRef] [Scilit]
- Barlag, B.; Hensel, M. The giant adhesin SiiE of Salmonella enterica. Molecules 2015, 20, 1134–1150. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ménard, S.; Lacroix-Lamandé, S.; Ehrhardt, K.; Yan, J.; Grassl, G.A.; Wiedemann, A. Cross-talk between the intestinal epithelium and Salmonella Typhimurium. Front. Microbiol. 2022, 13, 906238. [Google Scholar] [CrossRef] [Scilit]
- Li, Q. Mechanisms for the invasion and dissemination of Salmonella. Can. J. Infect. Dis. Med. Microbiol. 2022, 2022, 2655801. [Google Scholar] [CrossRef] [Scilit]
- Worley, M.J. Immune evasion and persistence in enteric bacterial pathogens. Gut Microbes 2023, 15, 2163839. [Google Scholar] [CrossRef] [Scilit]
- Li, Y.; Xu, Y.; Jin, C.; Qiu, J.; Jiao, X.; Pan, Z.; Guo, Y. Salmonella–NLRP3 inflammasome crosstalk: Host defense activation versus bacterial immune evasion strategies. J. Inflamm. Res. 2025, 18, 5133–5148. [Google Scholar] [CrossRef] [Scilit]
- Allen, J.C.; Natta, S.S.; Nasrin, S.; Toapanta, F.R.; Tennant, S.M. Deletion of an immune evasion gene, steD, from a live Salmonella enterica serotype Typhimurium vaccine improves vaccine responses in aged mice. Front. Immunol. 2024, 15, 1376734. [Google Scholar] [CrossRef] [Scilit]
- Grote, A.; Hendin, N.; Amit, S.; Adani, B.; Rahav, G.; Adler, A.; Livny, J.; Gal-Mor, O.; Earl, A.M. Genetic diversity of Salmonella enterica during acute human infections. Gut Microbes 2025, 17, 2491666. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jones, T.F.; Ingram, L.A.; Cieslak, P.R.; Vugia, D.J.; Tobin-D’Angelo, M.; Hurd, S.; Medus, C.; Cronquist, A.; Angulo, F.J. Salmonellosis outcomes differ substantially by serotype. J. Infect. Dis. 2008, 198, 109–114. [Google Scholar] [CrossRef] [Scilit]
- Harvey, R.R.; Friedman, C.R.; Crim, S.M.; Judd, M.; Barrett, K.A.; Tolar, B.; Folster, J.P.; Griffin, P.M.; Brown, A.C. Epidemiology of Salmonella enterica serotype Dublin infections among humans, United States, 1968–2013. Emerg. Infect. Dis. 2017, 23, 1493–1501. [Google Scholar] [CrossRef] [Scilit]
- Zhang, L.F.; Lepenies, B.; Nakamae, S.; Young, B.M.; Santos, R.L.; Raffatellu, M.; Cobb, B.A.; Hiyoshi, H.; Bäumler, A.J. The Vi capsular polysaccharide of Salmonella Typhi promotes macrophage phagocytosis by binding the human C-type lectin DC-SIGN. mBio 2022, 13, e02733-22. [Google Scholar] [CrossRef] [Scilit]
- Wangdi, T.; Lee, C.Y.; Spees, A.M.; Yu, C.; Kingsbury, D.D.; Winter, S.E.; Hastey, C.J.; Wilson, R.P.; Heinrich, V.; Bäumler, A.J. The Vi capsular polysaccharide enables Salmonella enterica serotype Typhi to evade microbe-guided neutrophil chemotaxis. PLoS Pathog. 2014, 10, e1004306. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chu, C.; Chiu, C.H. Evolution of the virulence plasmids of non-typhoid Salmonella and its association with antimicrobial resistance. Microbes Infect. 2006, 8, 1931–1936. [Google Scholar] [CrossRef] [Scilit]
- Schwan, W.R.; Huang, X.Z.; Hu, L.; Kopecko, D.J. Differential bacterial survival, replication, and apoptosis-inducing ability of Salmonella serotypes within human and murine macrophages. Infect. Immun. 2000, 68, 1005–1013. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kushwaha, S.K.; Wu, Y.; Leonardo Avila, H.; Anand, A.; Sicheritz-Pontén, T.; Millard, A.; Amol Marathe, S.; Nobrega, F.L. Comprehensive blueprint of Salmonella genomic plasticity identifies hotspots for pathogenicity genes. PLoS Biol. 2024, 22, e3002746. [Google Scholar] [CrossRef] [Scilit]
- Juhas, M.; van der Meer, J.R.; Gaillard, M.; Harding, R.M.; Hood, D.W.; Crook, D.W. Genomic islands: Tools of bacterial horizontal gene transfer and evolution. FEMS Microbiol. Rev. 2009, 33, 376–393. [Google Scholar] [CrossRef] [Scilit]
- Wahl, A.; Battesti, A.; Ansaldi, M. Prophages in Salmonella enterica: A driving force in reshaping the genome and physiology of their bacterial host. Mol. Microbiol. 2019, 111, 303–316. [Google Scholar] [CrossRef] [Scilit]
- Lerminiaux, N.A.; MacKenzie, K.D.; Cameron, A.D.S. Salmonella pathogenicity island 1 (SPI-1): The evolution and stabilization of a core genomic type III secretion system. Microorganisms 2020, 8, 576. [Google Scholar] [CrossRef] [Scilit]
- Lou, L.; Zhang, P.; Piao, R.; Wang, Y. Salmonella pathogenicity island 1 (SPI-1) and its complex regulatory network. Front. Cell. Infect. Microbiol. 2019, 9, 270. [Google Scholar] [CrossRef] [Scilit]
- Seth-Smith, H.M.; Fookes, M.C.; Okoro, C.K.; Baker, S.; Harris, S.R.; Scott, P.; Pickard, D.; Quail, M.A.; Churcher, C.; Sanders, M.; et al. Structure, diversity, and mobility of the Salmonella pathogenicity island 7 family of integrative and conjugative elements within Enterobacteriaceae. J. Bacteriol. 2012, 194, 1494–1504. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, W.; Fang, T.; Zhou, X.; Zhang, D.; Shi, X.; Shi, C. IncHI2 plasmids are predominant in antibiotic-resistant Salmonella isolates. Front. Microbiol. 2016, 7, 1566. [Google Scholar] [CrossRef] [Scilit]
- Finn, S.; Condell, O.; McClure, P.; Amézquita, A.; Fanning, S. Mechanisms of survival, responses, and sources of Salmonella in low-moisture environments. Front. Microbiol. 2013, 4, 331. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Aleksandrowicz, A.; Carolak, E.; Dutkiewicz, A.; Błachut, A.; Waszczuk, W.; Grzymajlo, K. Better together—Salmonella biofilm-associated antibiotic resistance. Gut Microbes 2023, 15, 2229937. [Google Scholar] [CrossRef] [Scilit]
- Pilch, H.; Aulik, N.; Sockett, D.; Czuprynski, C.J. Survival of bovine-associated serotypes of Salmonella enterica in bedding sand. JDS Commun. 2022, 4, 86–90. [Google Scholar] [CrossRef] [Scilit]
- Waldner, L.L.; MacKenzie, K.D.; Köster, W.; White, A.P. From exit to entry: Long-term survival and transmission of Salmonella. Pathogens 2012, 1, 128–155. [Google Scholar] [CrossRef] [Scilit]
- Krüger, G.I.; Urbina, F.; Pardo-Esté, C.; Salinas, V.; Álvarez, J.; Avilés, N.; Oviedo, A.; Kusch, C.; Pavez, V.; Vernal, R.; et al. Resilient by design: Environmental stress promotes biofilm formation and multi-resistance in poultry-associated Salmonella. Microorganisms 2025, 13, 1812. [Google Scholar] [CrossRef] [Scilit]
- Ajmera, A.; Shabbir, N. Salmonella. In StatPearls; StatPearls Publishing: Treasure Island, FL, USA, 2023. [Google Scholar]
- Wang, Y.; Xu, X.; Jia, S.; Qu, M.; Pei, Y.; Qiu, S.; Zhang, J.; Liu, Y.; Ma, S.; Lyu, N.; et al. A global atlas and drivers of antimicrobial resistance in Salmonella during 1900–2023. Nat. Commun. 2025, 16, 4611. [Google Scholar] [CrossRef] [Scilit]
- Peruzy, M.F.; Murru, N.; Carullo, M.R.; La Tela, I.; Rippa, A.; Balestrieri, A.; Proroga, Y.T.R. Antibiotic-resistant Salmonella circulation in the human population in the Campania region (2010–2023). Antibiotics 2025, 14, 189. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Crump, J.A.; Nyirenda, T.S.; Kalonji, L.M.; Phoba, M.F.; Tack, B.; Platts-Mills, J.A.; Gordon, M.A.; Kariuki, S.M. Nontyphoidal Salmonella invasive disease: Challenges and solutions. Open Forum Infect. Dis. 2023, 10, S32–S37. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Forgaciu, A.; Tabaran, A.; Colobatiu, L.; Mihaiu, R.; Dan, S.D.; Mihaiu, M. Concerning increase in antimicrobial resistance patterns of pathogenic strains of Salmonella isolated in poultry meat products. Antibiotics 2022, 11, 1469. [Google Scholar] [CrossRef] [Scilit]
- Niu, X.; Tu, L.; Yu, Q.; Lu, B.; Tian, J.; Wang, W.; Hou, B.; Shen, W. Serotypes and antimicrobial resistance patterns of food-borne Salmonella isolates in the Jiaxing region, China, from 2020 to 2024. J. Glob. Antimicrob. Resist. 2025, 45, 294–298. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Carey, M.E.; Dyson, Z.A.; Ingle, D.J.; Amir, A.; Aworh, M.K.; Chattaway, M.A.; Chew, K.L.; Crump, J.A.; Feasey, N.A.; Howden, B.P.; et al. Global diversity and antimicrobial resistance of typhoid fever pathogens. eLife 2023, 12, e85867. [Google Scholar] [CrossRef] [Scilit]
- François Watkins, L.K.; Winstead, A.; Appiah, G.D.; Friedman, C.R.; Medalla, F.; Hughes, M.J.; Birhane, M.G.; Schneider, Z.D.; Marcenac, P.; Hanna, S.S.; et al. Update on extensively drug-resistant Salmonella serotype Typhi infections among travelers to or from Pakistan and report of ceftriaxone-resistant Salmonella serotype Typhi infections among travelers to Iraq—United States, 2018–2019. MMWR Morb. Mortal. Wkly. Rep. 2020, 69, 618–622. [Google Scholar] [CrossRef] [Scilit]
- Sati, H.; Carrara, E.; Savoldi, A.; Hansen, P.; Garlasco, J.; Campagnaro, E.; Boccia, S.; Castillo-Polo, J.A.; Magrini, E.; Garcia-Vello, P.; et al. The WHO bacterial priority pathogens list 2024: A prioritisation study to guide research, development, and public health strategies against antimicrobial resistance. Lancet Infect. Dis. 2025, 25, 1033–1043. [Google Scholar] [CrossRef] [Scilit]
- Yoon, K.B.; Song, B.J.; Shin, M.Y.; Lim, H.C.; Yoon, Y.H.; Jeon, D.Y.; Ha, H.; Yang, S.I.; Kim, J.B. Antibiotic resistance patterns and serotypes of Salmonella spp. isolated at Jeollanam-do in Korea. Osong Public Health Res. Perspect. 2017, 8, 211–219. [Google Scholar] [CrossRef] [Scilit]
- Phaophu, P.; Thadtapong, N.; Wirth, S.E.; Gray, A.S.; Dangsuk, S.; Ngamwongsatit, N.; Aunpad, R.; Chaturongakul, S. High prevalence of multidrug-resistant Salmonella enterica in Thailand food markets. Microbiol. Spectr. 2025, 13, e02129-25. [Google Scholar] [CrossRef] [Scilit]
- Masuet-Aumatell, C.; Atouguia, J. Typhoid fever infection—Antibiotic resistance and vaccination strategies: A narrative review. Travel Med. Infect. Dis. 2021, 40, 101946. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Plumb, I.D.; Brown, A.C.; Stokes, E.K.; Chen, J.C.; Carleton, H.; Tolar, B.; Sundararaman, P.; Saupe, A.; Payne, D.C.; Shah, H.J.; et al. Increased multidrug-resistant Salmonella enterica I 4,[5],12:i:- infections associated with pork, United States, 2009–2018. Emerg. Infect. Dis. 2023, 29, 314–322. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jeong, J.; Chae, M.; Kang, M.-S.; Lee, J.-Y.; Kwon, Y.-K.; Lee, H.-J.; Lee, S.-H.; Son, H.-B.; Moon, J.-S.; Cho, S. Emergence and characteristics of multidrug-resistant Salmonella enterica serotype Infantis harboring the pESI plasmid in chicken slaughterhouses in South Korea. Microbiol. Spectr. 2025, 13, e0295524. [Google Scholar] [CrossRef] [Scilit]
- Di Marcantonio, L.; Romantini, R.; Marotta, F.; Chiaverini, A.; Zilli, K.; Abass, A.; Di Giannatale, E.; Garofolo, G.; Janowicz, A. The current landscape of antibiotic resistance of Salmonella Infantis in Italy. Front. Microbiol. 2022, 13, 812481. [Google Scholar] [CrossRef] [Scilit]
- Garcia, C.; Hinostroza, N.; Astocondor, L.; Ochoa, T.; Jacobs, J. For The Salmoiber Cyted Network. Characterization of ESBL-producing Salmonella enterica serotype Infantis infection in humans, Lima, Peru. Am. J. Trop. Med. Hyg. 2019, 101, 746–748. [Google Scholar] [CrossRef] [Scilit]
- Marder, E.P.; Griffin, P.M.; Cieslak, P.R.; Dunn, J.; Hurd, S.; Jervis, R.; Lathrop, S.; Muse, A.; Ryan, P.; Smith, K.; et al. Preliminary incidence and trends of infections with pathogens transmitted commonly through food—FoodNet, United States, 2006–2017. MMWR Morb. Mortal. Wkly. Rep. 2018, 67, 324–328. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ford, L.; Ellison, Z.; Schwensohn, C.; Griffin, I.; Birhane, M.G.; Cote, A.; Fortenberry, G.Z.; Tecle, S.; Higa, J.; Spencer, S.; et al. Strain of multidrug-resistant Salmonella Newport remains linked to travel to Mexico and U.S. beef products—United States, 2021–2022. MMWR Morb. Mortal. Wkly. Rep. 2023, 72, 1225–1229. [Google Scholar] [CrossRef]
- McMillan, E.A.; Jackson, C.R.; Frye, J.G. Transferable plasmids of Salmonella enterica associated with antibiotic resistance genes. Front. Microbiol. 2020, 11, 562181. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Carattoli, A. Plasmid-mediated antimicrobial resistance in Salmonella enterica. Curr. Issues Mol. Biol. 2003, 5, 113–122. [Google Scholar] [CrossRef] [Scilit]
- Lee, K.E.; Lim, S.I.; Choi, H.W.; Lim, S.K.; Song, J.Y.; An, D.J. Plasmid-mediated AmpC β-lactamase (CMY-2) gene in Salmonella Typhimurium isolated from diarrheic pigs in South Korea. BMC Res. Notes 2014, 7, 329. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gay, K.; Robicsek, A.; Strahilevitz, J.; Park, C.H.; Jacoby, G.; Barrett, T.J.; Medalla, F.; Chiller, T.M.; Hooper, D.C. Plasmid-mediated quinolone resistance in non-Typhi serotypes of Salmonella enterica. Clin. Infect. Dis. 2006, 43, 297–304. [Google Scholar] [CrossRef] [Scilit]
- Strahilevitz, J.; Jacoby, G.A.; Hooper, D.C.; Robicsek, A. Plasmid-mediated quinolone resistance: A multifaceted threat. Clin. Microbiol. Rev. 2009, 22, 664–689. [Google Scholar] [CrossRef] [Scilit]
- Cuypers, W.L.; Jacobs, J.; Wong, V.; Klemm, E.J.; Deborggraeve, S.; Van Puyvelde, S. Fluoroquinolone resistance in Salmonella: Insights by whole-genome sequencing. Microb. Genom. 2018, 4, e000195. [Google Scholar] [CrossRef] [Scilit]
- de Souza, R.B.; Magnani, M.; Ferrari, R.G.; Kottwitz, L.B.; Sartori, D.; Tognim, M.C.; de Oliveira, T.C. Detection of quinolone-resistance mutations in Salmonella spp. Braz. J. Microbiol. 2011, 42, 211–215. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Papp-Wallace, K.M.; Endimiani, A.; Taracila, M.A.; Bonomo, R.A. Carbapenems: Past, present, and future. Antimicrob. Agents Chemother. 2011, 55, 4943–4960. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Day, M.R.; Meunier, D.; Doumith, M.; de Pinna, E.; Woodford, N.; Hopkins, K.L. Carbapenemase-producing Salmonella enterica isolates in the UK. J. Antimicrob. Chemother. 2015, 70, 2165–2167. [Google Scholar] [CrossRef] [Scilit]
- Fernández, J.; Guerra, B.; Rodicio, M.R. Resistance to carbapenems in non-typhoidal Salmonella enterica serovars from Humans, Animals and Food. Vet. Sci. 2018, 5, 40. [Google Scholar] [CrossRef] [Scilit]
- Hsu, P.-C.; Wang, Y.-W.; Chen, B.-H.; Hong, Y.-P.; Teng, R.-H.; Liu, P.-Y.; Chiou, C.-S. Carbapenem resistance in extensively drug-resistant Salmonella enterica serovar Agona and AmpC β-lactamase-producing S. Infantis. Microbiol. Spectr. 2023, 11, e0292223. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Song, H.; Zou, S.; Wang, Y.; Chen, Z.; Sun, Z.; Jian, C. Emergence of carbapenem-resistant Salmonella Mbandaka through IS26-driven blaNDM-1 mobilization and chromosomal structural variation. Microbiol. Spectr. 2025, 13, e0096725. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Alhumaidan, O.S. Comprehensive review of salmonellosis: Current status of the disease and future perspectives. Ital. J. Food Saf. 2024, 13, 12904. [Google Scholar] [CrossRef] [Scilit]
- Kim, C.; Frost, I.; Naylor, N.R.; Au, H.; Kim, Y.; Lee, Y.; Bzymek, A.; Majgier, K.; Moldoveanu, A.L.; Salman, O.M.; et al. Length of hospital stay and associated treatment costs for patients with susceptible and antibiotic-resistant Salmonella infections: A systematic review and meta-analysis. BMJ Open 2025, 15, e092494. [Google Scholar] [CrossRef] [Scilit]
- Al Kraiem, A.A.; Yang, G.; Al Kraiem, F.; Chen, T. Challenges associated with ceftriaxone resistance in Salmonella. Front Life Sci. 2018, 11, 26–34. [Google Scholar] [CrossRef] [Scilit]
- Ayman, M.M.; Rawezh, Q.S.; Hidayat, A.Y.; Wafa, A.H.; Suhaib, H.K.; Fakher, A.; Karokh, K.M.; Dyari, Q.H.; Brwa, H.I.; Hawnaz, S.A.; et al. Evolution of antimicrobial resistance in community versus hospital-acquired infections. Barw Med. J. 2024, 3. [Google Scholar] [CrossRef] [Scilit]
- World Health Organization. Global Antimicrobial Resistance Surveillance System (GLASS) Report; World Health Organization: Geneva, Switzerland, 2017. [Google Scholar]
- Maron, J.L. The importance of ongoing surveillance, education, and due diligence for antimicrobial stewardship. Clin. Ther. 2024, 46, 441. [Google Scholar] [CrossRef] [Scilit]
- McEwen, S.A.; Collignon, P.J. Antimicrobial resistance: A One Health perspective. Microbiol. Spectr. 2018, 6. [Google Scholar] [CrossRef] [Scilit]
- Foley, S.L.; Nayak, R.; Hanning, I.B.; Johnson, T.J.; Han, J.; Ricke, S.C. Population dynamics of Salmonella enterica serotypes in poultry production. Appl. Environ. Microbiol. 2011, 77, 4273–4279. [Google Scholar] [CrossRef] [Scilit]
- Dowd, S.E.; Sun, Y.; Wolcott, R.D.; Domingo, A.; Carroll, J.A. Bacterial tag-encoded flx amplicon pyrosequencing (btefap) for microbiome studies: Bacterial diversity in the ileum of newly weaned Salmonella-infected pigs. Foodborne Pathog. Dis. 2008, 5, 459–472. [Google Scholar] [CrossRef] [Scilit]
- Eng, S.K.; Pusparajah, P.; Ab Mutalib, N.S.; Ser, H.L.; Chan, K.G.; Lee, L.H. Salmonella: Pathogenesis and antibiotic resistance. Front. Life Sci. 2015, 8, 284–293. [Google Scholar] [CrossRef] [Scilit]
- Food and Drug Administration; Centers for Disease Control and Prevention; U.S. Department of Agriculture. National Antimicrobial Resistance Monitoring System (NARMS) Integrated Report; U.S. Food and Drug Administration: Silver Spring, MD, USA, 2021.
- Amato, L.; Benedetti, G.; Di Giuseppe, P.; Hénaux, V.; Lailler, R.; Nordeng, Z.; Scharffenberg, T.A.Z.; Skjerdal, T.; Cito, F. Mapping food surveillance chains through different sectors. Front. Public Health 2023, 11, 1129851. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mermin, J.; Hutwagner, L.; Vugia, D.; Shallow, S.; Daily, P.; Bender, J.; Koehler, J.; Marcus, R.; Angulo, F.J. Reptiles, Amphibians, and human Salmonella infection: A Population-Based, Case-Control Study. Clin. Infect. Dis. 2004, 38, S253–S261. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lefebvre, S.L.; Reid-Smith, R.; Boerlin, P.; Weese, J.S. Evaluation of the risks of shedding Salmonellae and other potential pathogens by therapy dogs fed raw diets in Ontario and Alberta. Zoonoses Public Health 2008, 55, 470–480. [Google Scholar] [CrossRef] [Scilit]
- Chen, M.H.; Hwang, W.Z.; Wang, S.W.; Shih, Y.C.; Tsen, H.Y. Pulsed field gel electrophoresis (pfge) analysis for multidrug resistant Salmonella enterica serovar schwarzengrund isolates collected in six years (2000–2005) from retail chicken meat in Taiwan. Food Microbiol. 2011, 28, 399–405. [Google Scholar] [CrossRef] [Scilit]
- Bennett, S.D.; Sodha, S.V.; Ayers, T.L.; Lynch, M.F.; Gould, L.H.; Tauxe, R.V. Produce-associated outbreaks, USA, 1998–2013. Epidemiol. Infect. 2018, 146, 1397–1406. [Google Scholar] [CrossRef] [Scilit]
- Winfield, M.D.; Groisman, E.A. Role of nonhost environments in Salmonella and E. coli. Appl. Environ. Microbiol. 2003, 69, 3687–3694. [Google Scholar] [CrossRef] [Scilit]
- Franz, E.; van Bruggen, A.H.C. Ecology of E. coli O157:H7 and Salmonella enterica in the Primary Vegetable Production Chain. Crit. Rev. Microbiol. 2008, 34, 143–161. [Google Scholar] [CrossRef] [Scilit]
- Semenza, J.C.; Herbst, S.; Rechenburg, A.; Suk, J.E.; Höser, C.; Schreiber, C.; Kistemann, T. Climate change impact assessment of food- and waterborne diseases. Crit. Rev. Environ. Sci. Technol. 2012, 42, 857–890. [Google Scholar] [CrossRef] [Scilit]
- Semenov, A.V.; van Bruggen, A.H.; van Overbeek, L.; Termorshuizen, A.J.; Semenov, A.M. Influence of temperature fluctuations on Escherichia coli O157:H7 and Salmonella enterica serovar Typhimurium in cow manure. FEMS Microbiol. Ecol. 2007, 60, 419–428. [Google Scholar] [CrossRef] [Scilit]
- Heuer, H.; Schmitt, H.; Smalla, K. Antibiotic resistance gene spread due to manure application on agricultural fields. Curr. Opin. Microbiol. 2011, 14, 236–243. [Google Scholar] [CrossRef] [Scilit]
- Schwaiger, K.; Schmied, E.M.; Bauer, J. Comparative analysis of antibiotic resistance characteristics of Gram-negative bacteria isolated from laying hens and eggs in conventional and organic keeping systems in Bavaria, Germany. Zoonoses Public Health 2008, 55, 331–341. [Google Scholar] [CrossRef] [Scilit]
- Jackson, B.R.; Griffin, P.M.; Cole, D.; Walsh, K.A.; Chai, S.J. Outbreak-associated Salmonella serotypes. Emerg. Infect. Dis. 2013, 19, 1239–1244. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- World Health Organization. Salmonella (Non-Typhoidal); World Health Organization: Geneva, Switzerland, 2018; Available online: https://www.who.int/news-room/fact-sheets/detail/salmonella-(non-typhoidal) (accessed on 27 February 2026).
- Giannella, R.A. Salmonella. In Medical Microbiology, 4th ed.; Chapter 21; Baron, S., Ed.; University of Texas Medical Branch at Galveston: Galveston, TX, USA, 1996. Available online: https://www.ncbi.nlm.nih.gov/books/NBK8435/ (accessed on 27 February 2026).
- Watkins, L.K.F.; Shih, D.C.; Dorough, L. Typhoid and paratyphoid fever. In CDC Yellow Book; Centers for Disease Control and Prevention: Atlanta, GA, USA, 2025. Available online: https://www.cdc.gov/yellow-book/hcp/travel-associated-infections-diseases/typhoid-and-paratyphoid-fever.html (accessed on 27 February 2026).
- Centers for Disease Control and Prevention. Clinical Overview of Salmonellosis; Centers for Disease Control and Prevention: Atlanta, GA, USA, 2024. Available online: https://www.cdc.gov/salmonella/hcp/clinical-overview/index.html (accessed on 27 February 2026).
- World Health Organization. Typhoid vaccines: WHO position paper, March 2018—Recommendations. Vaccine 2019, 37, 214–216. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Food and Agriculture Organization of the United Nations; World Health Organization. Measures for the Control of Non-Typhoidal Salmonella spp. in Poultry Meat: Meeting Report; Food and Agriculture Organization: Rome, Italy, 2023. [Google Scholar]
- Codex Alimentarius Commission. Guidelines for the Control of Campylobacter and Salmonella in Chicken Meat (CXG 78-2011); FAO: Rome, Italy; WHO: Geneva, Switzerland, 2011. [Google Scholar]
- Centers for Disease Control and Prevention. Salmonella Outbreak Linked To Eggs; Centers for Disease Control and Prevention: Atlanta, GA, USA, 2025. Available online: https://www.cdc.gov/salmonella/outbreaks/eggs-08-25/index.html (accessed on 27 February 2026).
- Centers for Disease Control and Prevention. Reptiles and Amphibians; Centers for Disease Control and Prevention: Atlanta, GA, USA, 2026. Available online: https://www.cdc.gov/healthy-pets/about/reptiles-and-amphibians.html (accessed on 27 February 2026).
- U.S. Food and Drug Administration. HACCP Principles & Application Guidelines; U.S. Food and Drug Administration: Silver Spring, MD, USA, 2022. Available online: https://www.fda.gov/food/hazard-analysis-critical-control-point-haccp/haccp-principles-application-guidelines (accessed on 27 February 2026).
- Codex Alimentarius Commission. General principles of food hygiene (CXC 1-1969); FAO: Rome, Italy, 2022. [Google Scholar]
- UK Health Security Agency. Public Health Operational Guidelines for Typhoid and Paratyphoid (Enteric Fever); UK Health Security Agency: London, UK, 2024. Available online: https://www.gov.uk/government/publications/typhoid-and-paratyphoid-public-health-operational-guidelines (accessed on 27 February 2026).
- Bhutta, Z.A.; Gaffey, M.F.; Crump, J.A.; Steele, D.; Breiman, R.F.; Mintz, E.D.; Black, R.E.; Luby, S.P.; Levine, M.M. Typhoid fever: Way forward. Am. J. Trop. Med. Hyg. 2018, 99, 89–96. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tennant, S.M.; MacLennan, C.A.; Simon, R.; Martin, L.B.; Khan, M.I. Nontyphoidal Salmonella disease: Current status of vaccine research and development. Vaccine 2016, 34, 2907–2910. [Google Scholar] [CrossRef] [Scilit]
- Centers for Disease Control and Prevention. Treatment of Salmonella Infection; Centers for Disease Control and Prevention: Atlanta, GA, USA, 2024. Available online: https://www.cdc.gov/salmonella/treatment/index.html (accessed on 27 February 2026).
- Srinivasan, M.; Sindhu, K.N.; Giri, S.; Kumar, N.; Mohan, V.R.; Grassly, N.C.; Kang, G. Salmonella Typhi shedding and household transmission by children with blood culture-confirmed typhoid fever in South India. J. Infect. Dis. 2021, 224, S593–S600. [Google Scholar] [CrossRef] [Scilit]
- Gunn, J.S.; Marshall, J.M.; Baker, S.; Dongol, S.; Charles, R.C.; Ryan, E.T. Salmonella chronic carriage: Epidemiology, diagnosis, and gallbladder persistence. Trends Microbiol. 2014, 22, 648–655. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Centers for Disease Control and Prevention. Appendix A: Type and Duration of Precautions Recommended for Selected Infections And Conditions; Centers for Disease Control and Prevention: Atlanta, GA, USA, 2025. Available online: https://www.cdc.gov/infection-control/hcp/isolation-precautions/appendix-a-type-duration.html (accessed on 27 February 2026).
- Gnanasekaran, S.; Jayaraj, V.; Yazhini, V.B.; Mohanraj, P.S.; Babu, C.; Rajendran, N.; Rajendran, V. A comprehensive evaluation of water, sanitation, and hygiene (WASH) in health facilities: A systematic review and meta-analysis. J. Hosp. Infect. 2024, 151, 116–130. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Centers for Disease Control and Prevention. PulseNet: Today and Beyond; Centers for Disease Control and Prevention: Atlanta, GA, USA, 2024. Available online: https://www.cdc.gov/pulsenet/php/anniversary/index.html (accessed on 27 February 2026).
- Centers for Disease Control and Prevention. PulseNet Next Generation Technology; Centers for Disease Control and Prevention: Atlanta, GA, USA, 2024. Available online: https://www.cdc.gov/pulsenet/hcp/about/next-gen-wgs.html (accessed on 27 February 2026).
- Centers for Disease Control and Prevention. About the National Antimicrobial Resistance Monitoring System (NARMS); Centers for Disease Control and Prevention: Atlanta, GA, USA, 2024. Available online: https://www.cdc.gov/narms/about/index.html (accessed on 27 February 2026).
- Centers for Disease Control and Prevention. Data and Reports: NARMS; Centers for Disease Control and Prevention: Atlanta, GA, USA, 2025. Available online: https://www.cdc.gov/narms/data/index.html (accessed on 27 February 2026).
- Centers for Disease Control and Prevention. Data Summary: Emerging Strain of Salmonella Typhi (REPJPP01); Centers for Disease Control and Prevention: Atlanta, GA, USA, 2025. Available online: https://www.cdc.gov/typhoid-fever/php/rep-strain/index.html (accessed on 27 February 2026).
- Allard, M.W.; Strain, E.; Melka, D.; Bunning, K.; Musser, S.M.; Brown, E.W.; Timme, R. Practical value of food pathogen traceability through building a whole-genome sequencing network and database. J. Clin. Microbiol. 2016, 54, 1975–1983. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Aladhadh, M. A review of modern methods for the detection of foodborne pathogens. Microorganisms 2023, 11, 1111. [Google Scholar] [CrossRef] [Scilit]
- Schadron, T.; van den Beld, M.; Mughini-Gras, L.; Franz, E. Use of whole-genome sequencing for surveillance and control of foodborne diseases: Status quo and quo vadis. Front. Microbiol. 2024, 15, 1460335. [Google Scholar] [CrossRef] [Scilit]
- National Human Genome Research Institute. The Cost of Sequencing a Human Genome; National Human Genome Research Institute: Bethesda, MD, USA, 2021. Available online: https://www.genome.gov/about-genomics/fact-sheets/Sequencing-Human-Genome-cost (accessed on 27 February 2026).
- Aarestrup, F.M.; Brown, E.W.; Detter, C.; Gerner-Smidt, P.; Gilmour, M.W.; Harmsen, D.; Hendriksen, R.S.; Hewson, R.; Heymann, D.L.; Johansson, K.; et al. Integrating genome-based informatics to modernize global disease monitoring, information sharing, and response. Emerg. Infect. Dis. 2012, 18, e1. [Google Scholar] [CrossRef] [Scilit]
- Uelze, L.; Becker, N.; Borowiak, M.; Busch, U.; Dangel, A.; Deneke, C.; Fischer, J.; Flieger, A.; Hepner, S.; Huber, I.; et al. Toward an integrated genome-based surveillance of Salmonella enterica in Germany. Front. Microbiol. 2021, 12, 626941. [Google Scholar] [CrossRef] [Scilit]
- Aarestrup, F.M.; Koopmans, M.G. Sharing data for global infectious disease surveillance and outbreak detection. Trends Microbiol. 2016, 24, 241–245. [Google Scholar] [CrossRef] [Scilit]
- Yoshida, C.E.; Kruczkiewicz, P.; Laing, C.R.; Lingohr, E.J.; Gannon, V.P.; Nash, J.H.; Taboada, E.N. The Salmonella in silico typing resource (SISTR): An open web-accessible tool for rapidly typing and subtyping draft Salmonella genome assemblies. PLoS ONE 2016, 11, e0147101. [Google Scholar] [CrossRef] [Scilit]
- Bayliss, S.C.; Locke, R.K.; Jenkins, C.; Chattaway, M.A.; Dallman, T.J.; Cowley, L.A. Rapid geographical source attribution of Salmonella enterica serovar Enteritidis genomes using hierarchical machine learning. eLife 2023, 12, e84167. [Google Scholar] [CrossRef] [Scilit]
- Coipan, C.E.; Dallman, T.J.; Brown, D.; Hartman, H.; van der Voort, M.; van den Berg, R.R.; Palm, D.; Kotila, S.; van Wijk, T.; Franz, E. Concordance of SNP- and allele-based typing workflows in the context of a large-scale international Salmonella enteritidis outbreak investigation. Microb. Genom. 2020, 6, e000318. [Google Scholar] [CrossRef] [Scilit]
- Saber, M.M.; Shapiro, B.J. Benchmarking bacterial genome-wide association study methods using simulated genomes and phenotypes. Microb. Genom. 2020, 6, e000337. [Google Scholar] [CrossRef] [Scilit]
- Franz, E.; Gras, L.M.; Dallman, T. Significance of whole genome sequencing for surveillance, source attribution, and microbial risk assessment of foodborne pathogens. Curr. Opin. Food Sci. 2016, 8, 74–79. [Google Scholar] [CrossRef] [Scilit]
- Fu, Y.; M’ikanatha, N.M.; Lorch, J.M.; Blehert, D.S.; Berlowski-Zier, B.; Whitehouse, C.A.; Li, S.; Deng, X.; Smith, J.C.; Shariat, N.W.; et al. Salmonella enterica serovar Typhimurium isolates from wild birds in the United States represent distinct lineages defined by bird type. Appl. Environ. Microbiol. 2022, 88, e01979-21. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Merlotti, A.; Manfreda, G.; Munck, N.; Hald, T.; Litrup, E.; Nielsen, E.M.; Remondini, D.; Pasquali, F. Network approach to source attribution of Salmonella enterica serovar Typhimurium and its monophasic variant. Front. Microbiol. 2020, 11, 1205. [Google Scholar] [CrossRef] [Scilit]
- Mughini-Gras, L.; Kooh, P.; Fravalo, P.; Augustin, J.C.; Guillier, L.; David, J.; Thébault, A.; Carlin, F.; Leclercq, A.; Jourdan-Da-Silva, N.; et al. Critical orientation in the jungle of currently available methods and types of data for source attribution of foodborne diseases. Front. Microbiol. 2019, 10, 2578. [Google Scholar] [CrossRef] [Scilit]
- den Bakker, H.C.; Allard, M.W.; Bopp, D.; Brown, E.W.; Fontana, J.; Iqbal, Z.; Kinney, A.; Limberger, R.; Musser, K.A.; Shudt, M.; et al. Rapid whole-genome sequencing for surveillance of Salmonella enterica serovar Enteritidis. Emerg. Infect. Dis. 2014, 20, 1306–1314. [Google Scholar] [CrossRef] [Scilit]
- Smith, J.C.; Siceloff, A.T.; Shirazi, S.M.; Bell, R.L.; Shariat, N.W. A two-year study of Salmonella in four natural watersheds highlights the need for increased environmental Salmonella surveillance. Appl. Environ. Microbiol. 2025, 91, e0177025. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cohen, E.; Azriel, S.; Auster, O.; Gal, A.; Mikhlin, S.; Crauwels, S.; Rahav, G.; Gal-Mor, O. A new Salmonella enterica serovar isolated from a wild sparrow presents a distinct genetic, metabolic, and virulence profile. Microbes Infect. 2024, 26, 105249. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Deaven, A.M.; Ferreira, C.M.; Reed, E.A.; Chen See, J.R.; Lee, N.A.; Almaraz, E.; Rios, P.C.; Marogi, J.G.; Lamendella, R.; Zheng, J.; et al. Salmonella genomics and population analyses reveal high inter- and intraserovar diversity in freshwater. Appl. Environ. Microbiol. 2021, 87, e02594-20. [Google Scholar] [CrossRef] [Scilit]
- Topalcengiz, Z.; McEgan, R.; Danyluk, M.D. Fate of Salmonella in central Florida surface waters and evaluation of EPA worst-case water as a standard medium. J. Food Prot. 2019, 82, 916–925. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Centers for Disease Control and Prevention. BEAM (Bacteria, Enterics, Amoeba, and Mycotics) Dashboard; U.S. Department of Health Human Services: Atlanta, GA, USA, 2026. Available online: https://www.cdc.gov/ncezid/dfwed/BEAM-dashboard.html (accessed on 27 February 2026).
- Benevides, V.P.; Saraiva, M.M.S.; Ferreira, V.A.; Funnicelli, M.I.G.; Rodrigues Alves, L.B.; Almeida, A.M.; Christensen, H.; Olsen, J.E.; Berchieri Junior, A. Unveiling the genomic landscape of understudied Salmonella enterica serovars from poultry and humans. Curr. Microbiol. 2025, 82, 279. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Karunarathna, R.; Liu, C.C.; Periyasamy, D.; Berg, A.; Ngeleka, M.; Trokhymchuk, A. Toward decentralization of Salmonella serotyping and risk assessment in poultry production environments with nanopore sequencing. Front. Microbiol. 2025, 16, 1669089. [Google Scholar] [CrossRef] [Scilit]
- Ding, Y.; Zwe, Y.H.; Chin, S.F.; Kohli, G.S.; Drautz-Moses, D.I.; Givskov, M.; Schlundt, J.; Schuster, S.C.; Yuk, H.G.; Yang, L. Characterization of a novel multidrug resistance plasmid pSGB23 isolated from Salmonella enterica serovar Saintpaul. Gut Pathog. 2018, 10, 49. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cheng, R.A.; Eade, C.R.; Wiedmann, M. Embracing diversity: Differences in virulence mechanisms, disease severity, and host adaptations contribute to the success of nontyphoidal Salmonella as a foodborne pathogen. Front. Microbiol. 2019, 10, 1368. [Google Scholar] [CrossRef] [Scilit]
- Coburn, B.; Grassl, G.A.; Finlay, B.B. Salmonella, the host and disease: A brief review. Immunol. Cell Biol. 2007, 85, 112–118. [Google Scholar] [CrossRef] [Scilit]
- Hong, W.; Yang, Z.; Wu, G.; Liu, C.; Wang, Y.; Liao, N. Integrating serotyping, MLST, and phenotypic data: Decoding the evolutionary drivers of Salmonella pathogenicity and drug resistance. Appl. Environ. Microbiol. 2025, 91, e0151125. [Google Scholar] [CrossRef] [Scilit]
- Nazir, J.; Manzoor, T.; Saleem, A.; Gani, U.; Bhat, S.S.; Khan, S.; Haq, Z.; Jha, P.; Ahmad, S.M. Combatting Salmonella: A focus on antimicrobial resistance and the need for effective vaccination. BMC Infect. Dis. 2025, 25, 84. [Google Scholar] [CrossRef] [Scilit]
- Pornsukarom, S.; Van Vliet, A.H.M.; Thakur, S. Whole-genome sequencing analysis of multiple Salmonella serovars provides insights into phylogenetic relatedness, antimicrobial resistance, and virulence markers across humans, food animals, and agricultural environments. BMC Genom. 2018, 19, 801. [Google Scholar] [CrossRef] [Scilit]
- Dieye, Y.; Hull, D.M.; Wane, A.A.; Harden, L.; Fall, C.; Sambe-Ba, B.; Seck, A.; Fedorka-Cray, P.J.; Thakur, S. Genomics of human and chicken Salmonella isolates in Senegal: Broilers as a source of antimicrobial resistance and potentially invasive nontyphoidal salmonellosis infections. PLoS ONE 2022, 17, e0266025. [Google Scholar] [CrossRef] [Scilit]
- Woh, P.Y.; Chen, Y.; Nurjadi, D. Bridging the phylodynamic antimicrobial resistance of Salmonella in Southeast Asia and Hong Kong through a One Health lens. Int. J. Food Microbiol. 2025, 443, 111431. [Google Scholar] [CrossRef] [Scilit]
- Muturi, P.; Mbae, C.; Kibet, E.; Njoroge, P.; Kavai, S.M.; Ideke, D.; Jepchirchir, J.; Gunn, J.S.; Kariuki, S. Antimicrobial resistance and biofilm formation in rarely reported Salmonella enterica serovars from patients presenting with gastroenteritis in Nairobi, Kenya. Front. Microbiol. 2025, 16, 1628784. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Elder, J.R.; Chiok, K.L.; Paul, N.C.; Haldorson, G.; Guard, J.; Shah, D.H. The Salmonella pathogenicity island 13 contributes to pathogenesis in streptomycin pre-treated mice but not in day-old chickens. Gut Pathog. 2016, 8, 16. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Souza, A.I.S.; Saraiva, M.M.S.; Casas, M.R.T.; Oliveira, G.M.; Cardozo, M.V.; Benevides, V.P.; Barbosa, F.O.; Freitas Neto, O.C.; Almeida, A.M.; Berchieri, A., Jr. High occurrence of β-lactamase-producing Salmonella Heidelberg from poultry origin. PLoS ONE 2020, 15, e0230676. [Google Scholar] [CrossRef] [Scilit] [PubMed]
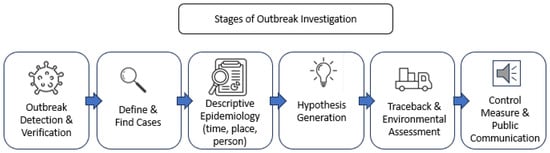

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.