Article

Sewage Sludge-Derived Biosolid and Bacillus aryabhattai as Bioinputs for Sustainable Sunflower Production

by
Laura Gonçalves Silva
,
Eduardo Ferreira de Almeida Santos
,
Alcindo Cravero Padilha
and
Inês Cechin
*
Department of Biological Science, UNESP-São Paulo State University, Av. Luiz Edimundo Carrijo Coube, 14-01, Bauru, São Paulo 17033-360, Brazil
*
Author to whom correspondence should be addressed.
Agronomy 2026, 16(8), 796; https://doi.org/10.3390/agronomy16080796
Submission received: 23 February 2026 / Revised: 8 April 2026 / Accepted: 8 April 2026 / Published: 13 April 2026
(This article belongs to the Section Farming Sustainability)

Abstract

Increasing domestic sewage production associated with urban population growth poses environmental challenges. Biosolids from wastewater treatment can recycle nutrients in agriculture, while plant growth-promoting rhizobacteria (PGPR) enhance nutrient availability and plant performance. This study evaluated the effects of the combined application of sewage sludge–derived biosolid and Bacillus aryabhattai on sunflower growth, biomass production, physiological traits, and nutrient status during the early growth stage under greenhouse conditions. We hypothesized that this combined treatment would enhance plant performance compared with biosolid application alone. Four treatments were established: control (T1), 5 g of biosolid alone (T2), 5 g biosolid + 3.2 mL B. aryabhattai (T3), and 5 g biosolid + 6.4 mL B. aryabhattai (T4). The formulation contains B. aryabhattai strain CMAA 1363 (1 × 10⁸ CFU mL−1) as the active microbial component, together with humic substances and other formulation agents (thickener, preservative, and water). The Plants were grown for 44 days. The data were analyzed using one-way ANOVA followed by mean comparison among treatments. Shoot dry mass was significantly higher in T4 compared with the T1 and T2 (p < 0.001), while no significant difference was observed between T3 and T4 (p > 0.05). Biosolid application increased the photosynthetic rate, and its combination with B. aryabhattai further enhanced photosynthetic performance, with significant difference detected between bacterial doses only at the end of growth period. Substomatal CO2 concentration was lower in inoculated treatments, indicating greater CO2 assimilation efficiency. Total chlorophyll increased with the addition of sludge and further increased by inoculation with 6.4 mL. Leaf N, Mn, and Zn contents were highest in T4. Overall, the combined application of biosolid and B. aryabhattai improved photosynthetic efficiency and biomass accumulation, highlighting the potential of integrating biosolids and beneficial rhizobacteria as a sustainable approach for nutrient recycling and improved crop productivity in agricultural systems.

1. Introduction

Increasing global food demand has intensified the need to increase agricultural productivity while reducing the environmental impacts associated with conventional fertilization practices. The excessive use of mineral fertilizers has raised concerns regarding soil degradation, nutrient leaching, and greenhouse gas emissions [1], highlighting the importance of more sustainable nutrient management strategies. In this context, organic amendments derived from waste recycling have gained increasing attention as alternatives capable of improving soil fertility while reducing dependence on synthetic inputs. Among these alternatives, biosolids generated during wastewater treatment represent a promising strategy for nutrient recycling in agriculture. These materials are generally rich in organic matter and essential plant nutrients and may improve soil physical, chemical, and biological properties [2,3]. Several studies have shown that biosolid application can enhance plant growth and crop productivity [4,5,6]. Thus, the agricultural reuse of biosolids may contribute to more sustainable production systems by returning nutrients from urban residues to agricultural soils.
In parallel, plant growth-promoting rhizobacteria (PGPR) have emerged as important biological tools for improving plant nutrition and performance. These microorganisms colonize plant roots and stimulate plant growth through multiple mechanisms, including phytohormone production, nutrient solubilization, and improved nutrient uptake efficiency [7]. Among PGPR, species of the genus Bacillus are particularly attractive because of their environmental resilience, rapid root colonization, and capacity to promote plant growth under a wide range of conditions [8,9,10,11]. In Brazil, B. aryabhattai has been found in the rhizosphere of Cereus jamacaru, an important cactus species native to the Caatinga biome [12] characterized by hot and semi-arid, with irregular rainfall and long dry periods. The species B. aryabhattai has received increasing attention because of its physiological versatility and its potential to enhance plant performance. Previous studies have shown that this bacterium can stimulate nutrient uptake, improve photosynthetic activity, and increase tolerance to abiotic stresses such as drought and salinity [9,13,14,15,16]. In addition, positive effects of B. aryabhattai on crop growth and productivity have been reported for maize, soybean, and sugarcane [17,18,19]. These attributes indicate that B. aryabhattai is a promising microbial bioinput for sustainable agriculture.
Despite the recognized benefits of biosolids and PGPR when applied separately, studies evaluating their combined use are still limited. Some recent studies have explored the association of B. aryabhattai with organic amendments such as vermicompost. For instance, Nguyen Van Chuong et al. [20] reported that the combined application of B. aryabhattai and vermicompost improved yield and nutrient uptake in peanut, indicating that this bacterium can act synergistically with organic nutrient sources. However, studies specifically addressing its combination with sewage sludge–derived biosolids remain scarce. A few studies reported that the incorporation of biosolids into the soil, associated with the inoculation of symbiotic microorganisms, promotes increased growth, photosynthetic pigment content, and improves soil fertility [21,22]. To the best of our knowledge, studies specifically investigating the combined application of biosolids and B. aryabhattai on plant growth remain scarce, and direct evidence for this combination is still limited. This limitation is particularly evident regarding their complementary effects on plant physiology, photosynthetic performance, and nutrient dynamics. Such a combination deserves further investigation because biosolids may serve as a nutrient-rich organic input, whereas PGPR may enhance nutrient mobilization, uptake, and physiological performance. Therefore, this study contributes to filling this knowledge gap by evaluating the combination of sewage sludge–derived biosolid with B. aryabhattai under controlled greenhouse conditions.
Sunflower (Helianthus annuus L.) is a crop of considerable agronomic and economic importance due to its adaptability and multiple uses, including oil production and crop rotation systems. In Brazil, sunflower cultivation has potential for further expansion, particularly in production regions such as the Cerrado [23]. In this context, identifying sustainable strategies capable of improving sunflower growth and physiology while reducing dependence on conventional fertilizers is of clear agronomic interest. The scientific novelty of this study lies in the evaluation of the combined application of sewage sludge–derived biosolid and B. aryabhattai, a combination that has been scarcely explored in the literature, particularly with respect to its effects on plant physiological performance and nutrient dynamics. While previous studies have investigated biosolids or PGPR separately, the potential complementary action between these two bioinputs remains poorly understood. In this context, this study provides new insights into whether biosolid and B. aryabhattai can act in a complementary manner to improve nutrient availability, photosynthetic performance, and biomass accumulation in sunflower. Specifically, we assessed the effects of their combined application on plant growth, shoot biomass production, leaf gas exchange, photosynthetic pigments, and nutrient content during the early growth stage under greenhouse conditions. We hypothesized that the combined application of sewage sludge–derived biosolid and B. aryabhattai enhances nutrient availability and uptake, resulting in increased photosynthetic activity, improved leaf nutrient status, and greater biomass accumulation compared with biosolid application alone.

2. Materials and Methods

2.1. Plant Material and Growth Conditions

Seeds of Helianthus annuus L. cv. Multissol were sown in pots with a maximum capacity of four liters, filled with Carolina Soil® (Carolina Soil do Brasil, Santa Cruz do Sul, Brazil) substrate mixed with medium-grade vermiculite at a 1:1 ratio (Carolina Soil®:vermiculite). The characteristics of pure Carolina substrate are shown in Table 1. This mixture diluted the available nutrients, reducing their concentration per unit volume, which can be interpreted as an approximate 50% reduction in the potential fertility of the substrate. The experiment was conducted in a greenhouse at the Department of Biological Sciences, UNESP–Bauru, under natural photoperiod conditions and without strict environmental control. The average minimum and maximum temperatures were 16 and 31 °C, respectively. One week after planting, thinning was carried out, leaving only one plant per pot. Irrigation with tap water was performed whenever necessary.

2.2. Application of Biosolid and Bacillus aryabhattai

The biosolid used in this study was kindly supplied by a certified company and produced for agricultural use in accordance with Brazilian environmental regulations (CONAMA Resolution No. 498/2020, classified as Class B), which establishes limits for heavy metals and other safety parameters in sewage sludge intended for agricultural application. Sabesfértil’s composition includes approximately 40% to 50% organic matter. Nutritional composition is presented in Table 2. The Sabesfértil biosolid, was applied on the day of sowing and then every 20 days until the end of the experiment. The biosolid was applied at a dose of 5 g per pot, corresponding to a field application rate of 1530.5 (kg ha−1).
The AURAS® inoculum formulation contains B. aryabhattai strain CMAA 1363 (1 × 10⁸ CFU mL−1) as the active microbial component, together with humic substances and other formulation agents (thickener, preservative, and water). The inoculant containing B. aryabhattai was applied at concentrations of 3.2 and 6.4 mL diluted in 100 mL of distilled water per pot. Inoculation was performed by incorporating the product into the substrate at the base of the plant, 10 days after sowing. Colonization was not directly assessed in this study. The plants were divided into four groups: T1: Substrate + 0 g of biosolids + 0 mL of B. aryabhattai; T2: Substrate + 5 g of biosolids + 0 mL of B. aryabhattai; T3: Substrate + 5 g of biosolids + 3.2 mL of B. aryabhattai; T4: Substrate + 5 g of biosolids + 6.4 mL of B. aryabhattai. The experiment followed a completely randomized design with four treatments, each consisting of 12 plants (48 plants in total). The number of plants randomly selected for each analysis is specified in the corresponding figure.

2.3. Growth Measurements

Growth measurements were performed weekly. Plant height was measured using a millimeter ruler, from the substrate surface to the last visible node. The number of emerged leaves was also recorded, with emerged leaves defined as those visible without handling the plant.

2.4. Measurements of Gas Exchange and Quantification of Photosynthetic Pigments

Photosynthetic rate (A), stomatal conductance (gs), and intercellular CO2 concentration (Ci) were measured using a portable open system infrared gas analyzer (LCpro, ADC BioScientific Ltd., Hoddesdon, UK). Measurements were performed on 10 plants per treatment at 23, 29, 36, and 42 days after sowing (DAS) using fully expanded leaves. Each pot was considered an experimental unit. Measurements were taken inside the greenhouse between 08:00 and 10:00 h under ambient conditions of temperature, CO2 partial pressure, and and air humidity, without environmental control of CO2 concentration, temperature, or relative humidity. The partial pressure of water vapor of the ambient air registered with the equipment ranged from 16.6 to 20.1 mBar between 08:00 and 10:00 h. A photosynthetically active radiation (PAR) of 800 μmol m−2 s−1 was provided by a light source (diode array containing blue LED at 470 nm and red ones at 660 nm. Between 5–10% of the photon are blue) attached to the leaf chamber. Leaves were maintained at this irradiance until steady-state photosynthetic rates were achieved. The A/Ci ratio was used to estimate instantaneous carboxylation efficiency, representing the amount of CO2 fixed during photosynthesis relative to its concentration in the intercellular air spaces.
For the quantification of photosynthetic pigments (chlorophylls and carotenoids), five independent plants per treatment were used for physiological measurements, with each pot considered an experimental unit. Three leaf discs per plant with a known area (1.68 cm2 each) were collected. The discs were homogenized in a mortar with 80% acetone, and pigment concentrations were calculated according to the equations proposed by Lichtenthaler [24]. Absorbance readings were obtained using a spectrophotometer (UV-1800; Shimadzu Corporation, Kyoto, Japan) at 647, 663, and 470 nm. Chlorophyll and carotenoid contents were expressed on a leaf area basis (g m−2).

2.5. Dry Mass Determination

At the end of the experimental period (44 days after sowing), plants from each treatment were harvested to determine shoot dry matter. Shoots were separated into stems and leaves and oven-dried at 65 °C for at least 48 h, or until constant mass was achieved. Dry matter was then determined using a precision balance.

2.6. Quantification of Macro and Micronutrient Content in Leaves and Biosolids

For nutrient analysis, mature leaves from representative plants from the median region from each treatment were collected and composited to obtain a representative sample, chemical analyses were performed in duplicate. The leaves were oven-dried in a forced-air circulation oven at 65 °C until constant weight was achieved. Subsequently, the samples were ground in a mill and, together with biosolid samples, sent to the Soil Laboratory of the Department of Soils and Environmental Resources, School of Agricultural Sciences, UNESP, Botucatu, for the determination of macro- and micronutrient contents according to the methodology described in the Manual of Official Analytical Methods for Fertilizers and Soil Amendments [25].

2.7. Statistical Analysis

Data were subjected to analysis of variance (ANOVA) according to a completely randomized design by using IBM SPSS Statistics 23 at a 5% significance level. Prior to the analysis, the assumptions of normality and homogeneity of variances were evaluated using the Shapiro–Wilk and Levene tests, respectively. When significant differences among treatments were detected by ANOVA (p  0.05 ), treatment means were compared using LSD test at the 5% probability level. The least significant difference (LSD) test was applied when variances were considered homogeneous, whereas the Games–Howell test was used when homogeneity of variances was not assumed. Statistical analyses of leaf number were performed after transforming the data using the equation x + 0.5 .

3. Results and Discussion

3.1. Nutrients

Antonkiewicz et al. [26] report that biowaste-derived materials can provide essential macro- and micronutrients for plant growth and promote improvements in soil physicochemical and biological properties. Domestic sewage sludge is characterized by high organic matter content, mainly composed of microbial biomass and particulate organic residues, whose composition and stability depend on the treatment process and directly affect its agronomic potential [27,28]. In the present study, the biosolid obtained after anaerobic digestion showed concentrations of P, S, Cu, Fe, Mn, and Zn above the optimal range for sunflower growth, whereas N, Mg, and K were slightly below the recommended levels, and Ca remained within the suitable range (Table 2). Despite the relatively high concentrations of Cu, Fe, Mn, and Zn in the biosolid, no increases in leaf concentrations or visual symptoms of toxicity were observed in sunflower plants. This finding suggests that the availability of these elements may be moderated by soil interactions or plant physiological regulation, preventing excessive accumulation in plant tissues. Consequently, biosolids may contain relatively high total concentrations of Fe, Mn, or Zn without necessarily causing toxicity in plant leaves, as observed in the present experiment. These results support the potential use of biosolids as a nutrient source in agricultural systems while highlighting that nutrient availability, rather than total concentration alone, plays a key role in determining plant responses.
The higher Fe content in domestic sewage results from a combination of human waste, household products, infrastructure corrosion, and the water supply itself, whereas elevated Zn concentrations are mainly associated with the widespread use of Zn-containing personal care products, detergents, and cleaning agents. Plants grown in biosolid-amended substrates exhibited higher leaf contents of N, K, Ca, Mg, S, Mn, and Zn compared with plants cultivated without biosolid application, indicating that the biosolid acted as an effective source of both macro- and micronutrients and enhanced nutrient availability and uptake (Table 2). Despite the high concentrations of Cu, Fe, Mn, and Zn in the biosolid relative to the optimal levels for sunflower, only Mn and Zn increased in the leaves compared with the control treatment. In contrast, leaf Fe concentrations decreased, which may be related to Zn-induced inhibition of Fe uptake and translocation [29]. A similar pattern was observed in the treatment combining biosolid with B. aryabhattai (T4), where leaf Zn increased from 45.5 to 70.0, whereas Fe decreased from 161 to 121 compared with the biosolid-only treatment (T1). Consequently, the Zn/Fe ratio increased from 0.28 to 0.58, indicating a shift in foliar micronutrient balance toward a relative enrichment in Zn. This result suggests that bacterial inoculation may have enhanced Zn availability and/or uptake through rhizosphere-mediated mechanisms.
Table 2. Nutrient content of pure Carolina Soil® substrate and leaves of sunflower plants. The analysis was done in duplicate. -, this symbol on the table means not determined. T1: Substrate + 0 g of biosolids + 0 mL of B. aryabhattai; T2: Substrate + 5 g of biosolids + 0 mL of B. aryabhattai; T3: Substrate + 5 g of biosolids + 3.2 mL of B. aryabhattai; T4: Substrate + 5 g of biosolids + 6.4 mL of B. aryabhattai.
VariablesMacronutrients (g Kg−1)Micronutrients (mg Kg−1)
N P K Ca Mg S B Cu Fe Mn Zn
Biosolid28.731.61.016.22.715.7-167.047,629.1279.5702.5
Suitable range for sunflower 130–503–530–458–223–81.5–2.0-25–10080–12010–2030–80
T132.24.545.212.88.64.339.720.0161.045.545.5
T239.94.650.413.59.96.255.019.5121.061.048.5
T340.24.749.410.99.15.047.923.0113.574.057.5
T443.74.948.810.48.75.245.421.5121.077.070.0
1 Adapted from [30,31].
B. aryabhattai has been reported to increase the availability of P, N and K in mung bean and maize crops [10]. In the present study, inoculation with B. aryabhattai combined with biosolid application increased leaf concentrations of N, Cu, Mn, and Zn, suggesting enhanced availability and uptake of these nutrients compared with non-inoculated leaves. In contrast, slight reductions in K, Ca, Mg, S, and B were observed, possibly reflecting nutrient interactions or dilution effects associated with increased leaf biomass production. Previous studies have shown that B. aryabhattai enhances the availability of micronutrients such as Cu, Mn and Zn [9,16,32] through mechanisms including nutrient solubilization, siderophore production, and rhizosphere modification. It has also been reported that high P concentrations may increase Zn adsorption due to the formation of P–Zn complexes on colloidal surfaces, potentially affecting Zn mobility in soil [33]. Compounds produced by B. aryabhattai can counteract such interactions by promoting Zn solubilization and availability [9]. The results suggest that the combined application of sewage sludge–derived biosolid and B. aryabhattai may influence plant performance through complementary mechanisms.
Biosolids represent an important source of macro- and micronutrients, whereas plant growth-promoting rhizobacteria can enhance nutrient mobilization and uptake through mechanisms such as phosphate solubilization, organic acid production, and siderophore-mediated micronutrient mobilization as pointed out by several authors [9,16,32]. The observed changes in leaf nutrient concentrations, particularly for elements associated with photosynthetic metabolism such as N, Mn and Zn, were consistent with the improvements in photosynthetic parameters and shoot biomass observed in inoculated plants. These results suggest that the combined use of biosolids and PGPR may contribute to improved nutrient use efficiency and physiological performance in sunflower. It is important to acknowledge a methodological limitation of the present study regarding the chemical analyses, which were performed in duplicate. Although this approach allowed the identification of consistent trends among treatments, the limited number of replicates may reduce the robustness and statistical reliability of the nutrient data. Therefore, the results should be interpreted with due caution, and future studies including a greater number of analytical replicates are recommended to improve the accuracy and reproducibility of the measurements.

3.2. Gas Exchange

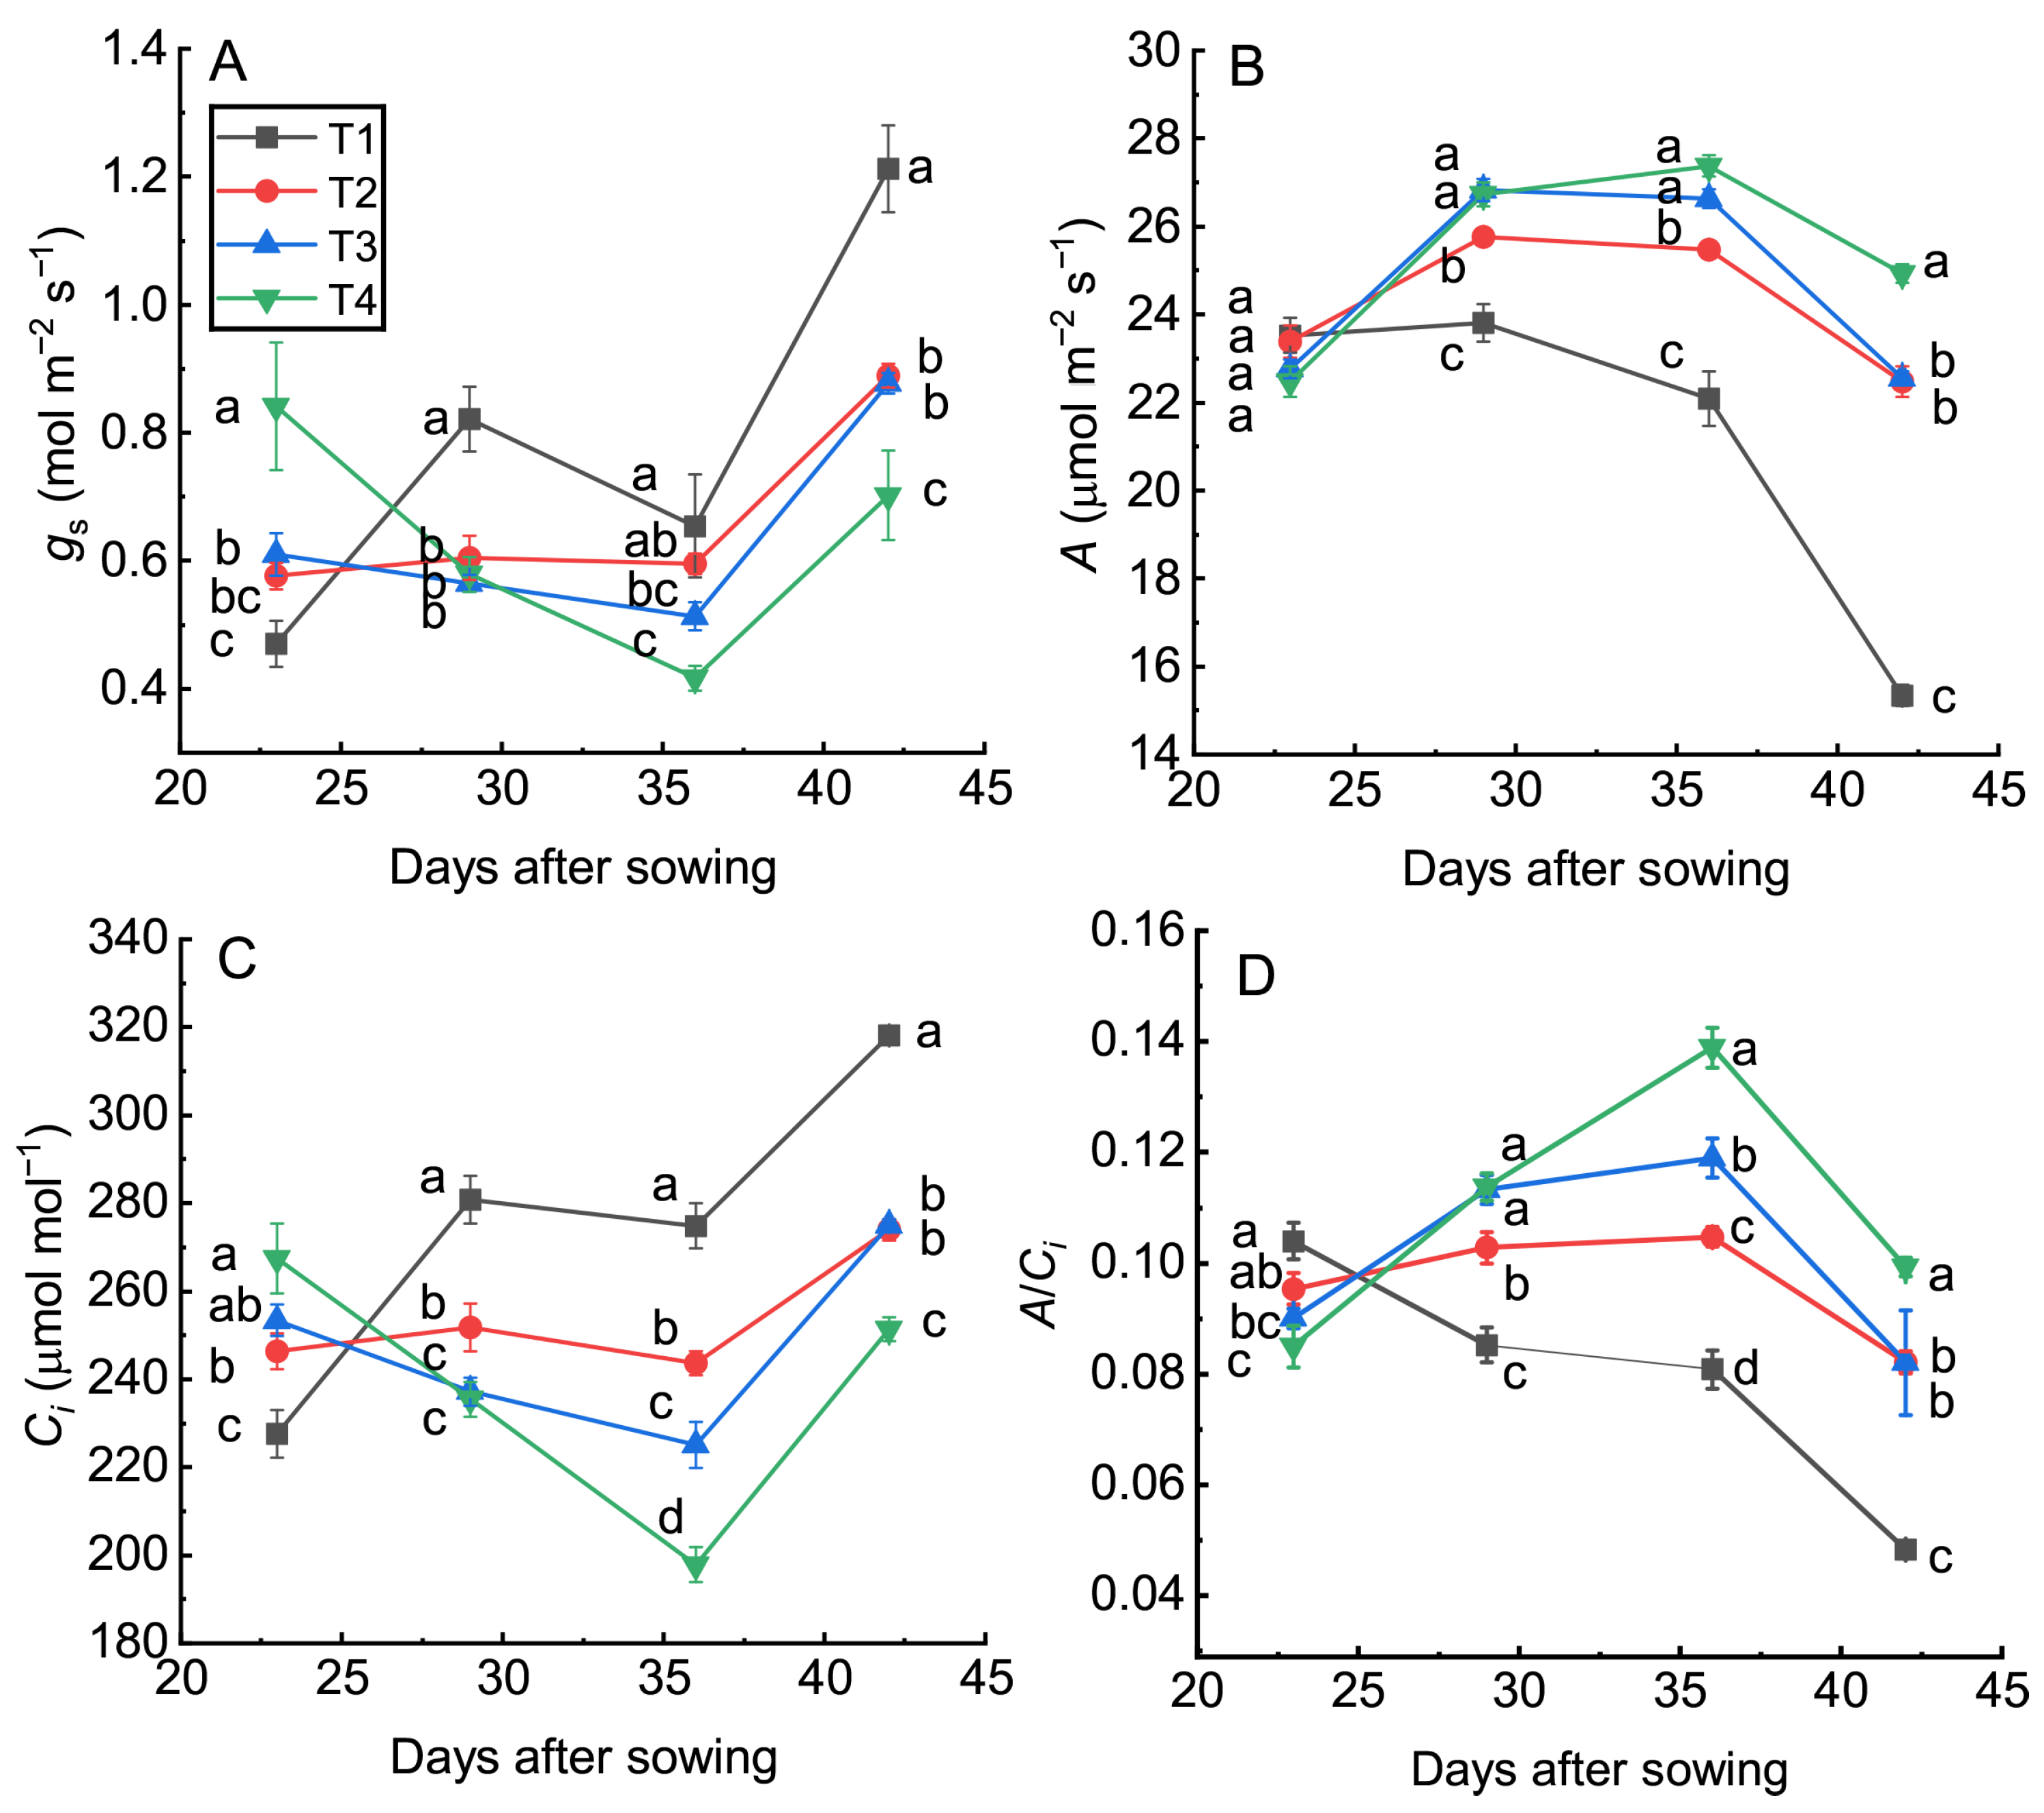
During the analysis of gas exchange, a considerable variation was observed in stomatal conductance rate (Figure 1A). The addition of biosolid in the substrate resulted in lower gs on 29 and 42 days after sowing compared with the plants without biosolid (Figure 1A). The inoculation with 6.4 mL of B. aryabhattai combined with biosolid application showed an increase in gs after 23 and a decrease 36 days of inoculation compared with no inoculation.
Photosynthetic capacity plays a central role in carbon assimilation efficiency and serves as an integrative indicator of plant responses to nutrient availability, thereby providing insight into the balance between nutrient demand and supply. Under the exclusive application of biosolid, a significant increase in photosynthetic rate was observed from 29 days after sowing compared with the no-addition treatment (Figure 1B), a trend that was also reported by Antolín et al. [34]. However, when biosolid was combined with B. aryabhattai, the increase was greater than that achieved with biosolid alone, with no significant difference between the two doses applied. At the end of the experiment, the photosynthetic rate of the plants receiving the lower dose of B. aryabhattai did not differ from that of non-inoculated plants. In contrast, under the higher B. aryabhattai dose, photosynthesis was significantly higher than in all other treatments. These results indicate that application of the higher B. aryabhattai dose was more effective in enhancing the plants’ capacity for CO2 fixation.
Intercellular CO2 concentration provides insight into the balance between CO2 diffusion and biochemical fixation; thus, increased Ci associated with reduced photosynthesis indicates non-stomatal limitations, whereas lower Ci coupled with higher assimilation reflects enhanced carboxylation efficiency. Plants grown without biosolid and B. aryabhattai exhibited higher Ci than those under the other treatments throughout the entire growth period (Figure 1C), which was accompanied by lower photosynthetic rates. In contrast, B. aryabhattai inoculation resulted in reduced Ci relative to non-inoculated plants, indicating enhanced CO2 fixation efficiency. These responses may be related to physiological mechanisms reported in the literature, including potential effects on Rubisco activity and non-stomatal limitations to photosynthesis [35,36,37]. Plants treated with the higher B. aryabhattai dose maintained lower Ci values together with higher photosynthetic rates, indicating improved CO2 fixation efficiency and highlighting the beneficial interaction between biosolid application and B. aryabhattai. The combined application of biosolid and B. aryabhattai enhanced photosynthetic rates while reducing Ci, suggesting improved carbon assimilation predominantly driven by non-stomatal limitations and increased carboxylation efficiency. This response may be partially explained by enhanced nutrient availability—particularly N, Cu, Mn, and Zn—and may also be associated with increased Rubisco expression by the biopriming technology, as reported by [38].
Throughout the sampling period, a marked decrease in carboxylation efficiency was observed, particularly in control plants without biosolid and B. aryabhattai, as the plants reached more advanced developmental stages and entered the reproductive phase (Figure 1D). During this phase, plants experience higher energetic demands associated with the formation of inflorescence and seeds. The reduction in photosynthetic capacity in older leaves is commonly linked to the active export of nutrients and assimilates to developing reproductive structures as observed by Kitajama [39], accelerating leaf senescence and limiting carbon fixation. Nevertheless, even under these conditions, the treatment with the highest dose of B. aryabhattai maintained superior performance, indicating enhanced efficiency in biosolid utilization when combined with bacterial inoculation. This response was likely associated with higher leaf nitrogen concentrations compared to the other treatments, supporting sustained carboxylation capacity during the reproductive stage.
B. aryabhattai has recently gained attention for its ability to enhance photosynthetic activity and nutrient uptake in other crops [40]. The increase in photosynthetic rate observed under the combined biosolid and B. aryabhattai treatment is likely associated with the greater availability of key nutrients provided by both the biosolid and bacterial activity, particularly N, Mg, Mn, and Zn, which support Rubisco content, chlorophyll synthesis, and enzymatic activation. Egamberdieva et al. [41] presented a comprehensive review demonstrating how microbial auxins, cytokinins, and gibberellins enhance photosynthetic capacity. Consistently, B. aryabhattai strains have been shown to synthesize several phyto-hormones, including auxins, giberellins, and abscisic acid [8,42]. Park et al. [8] further reported that the plants inoculated with B. aryabhattai strains maintained stable phytohormone levels, supporting the role of this bacterium in regulating plant physiological performance. Moreover, this treatment appears to mitigate the decline in photosynthesis typically observed during advanced developmental stages by sustaining source strength and optimizing source–sink relationships, thereby promoting more efficient carbon assimilation even during the reproductive phase.

3.3. Photosynthetic Pigments

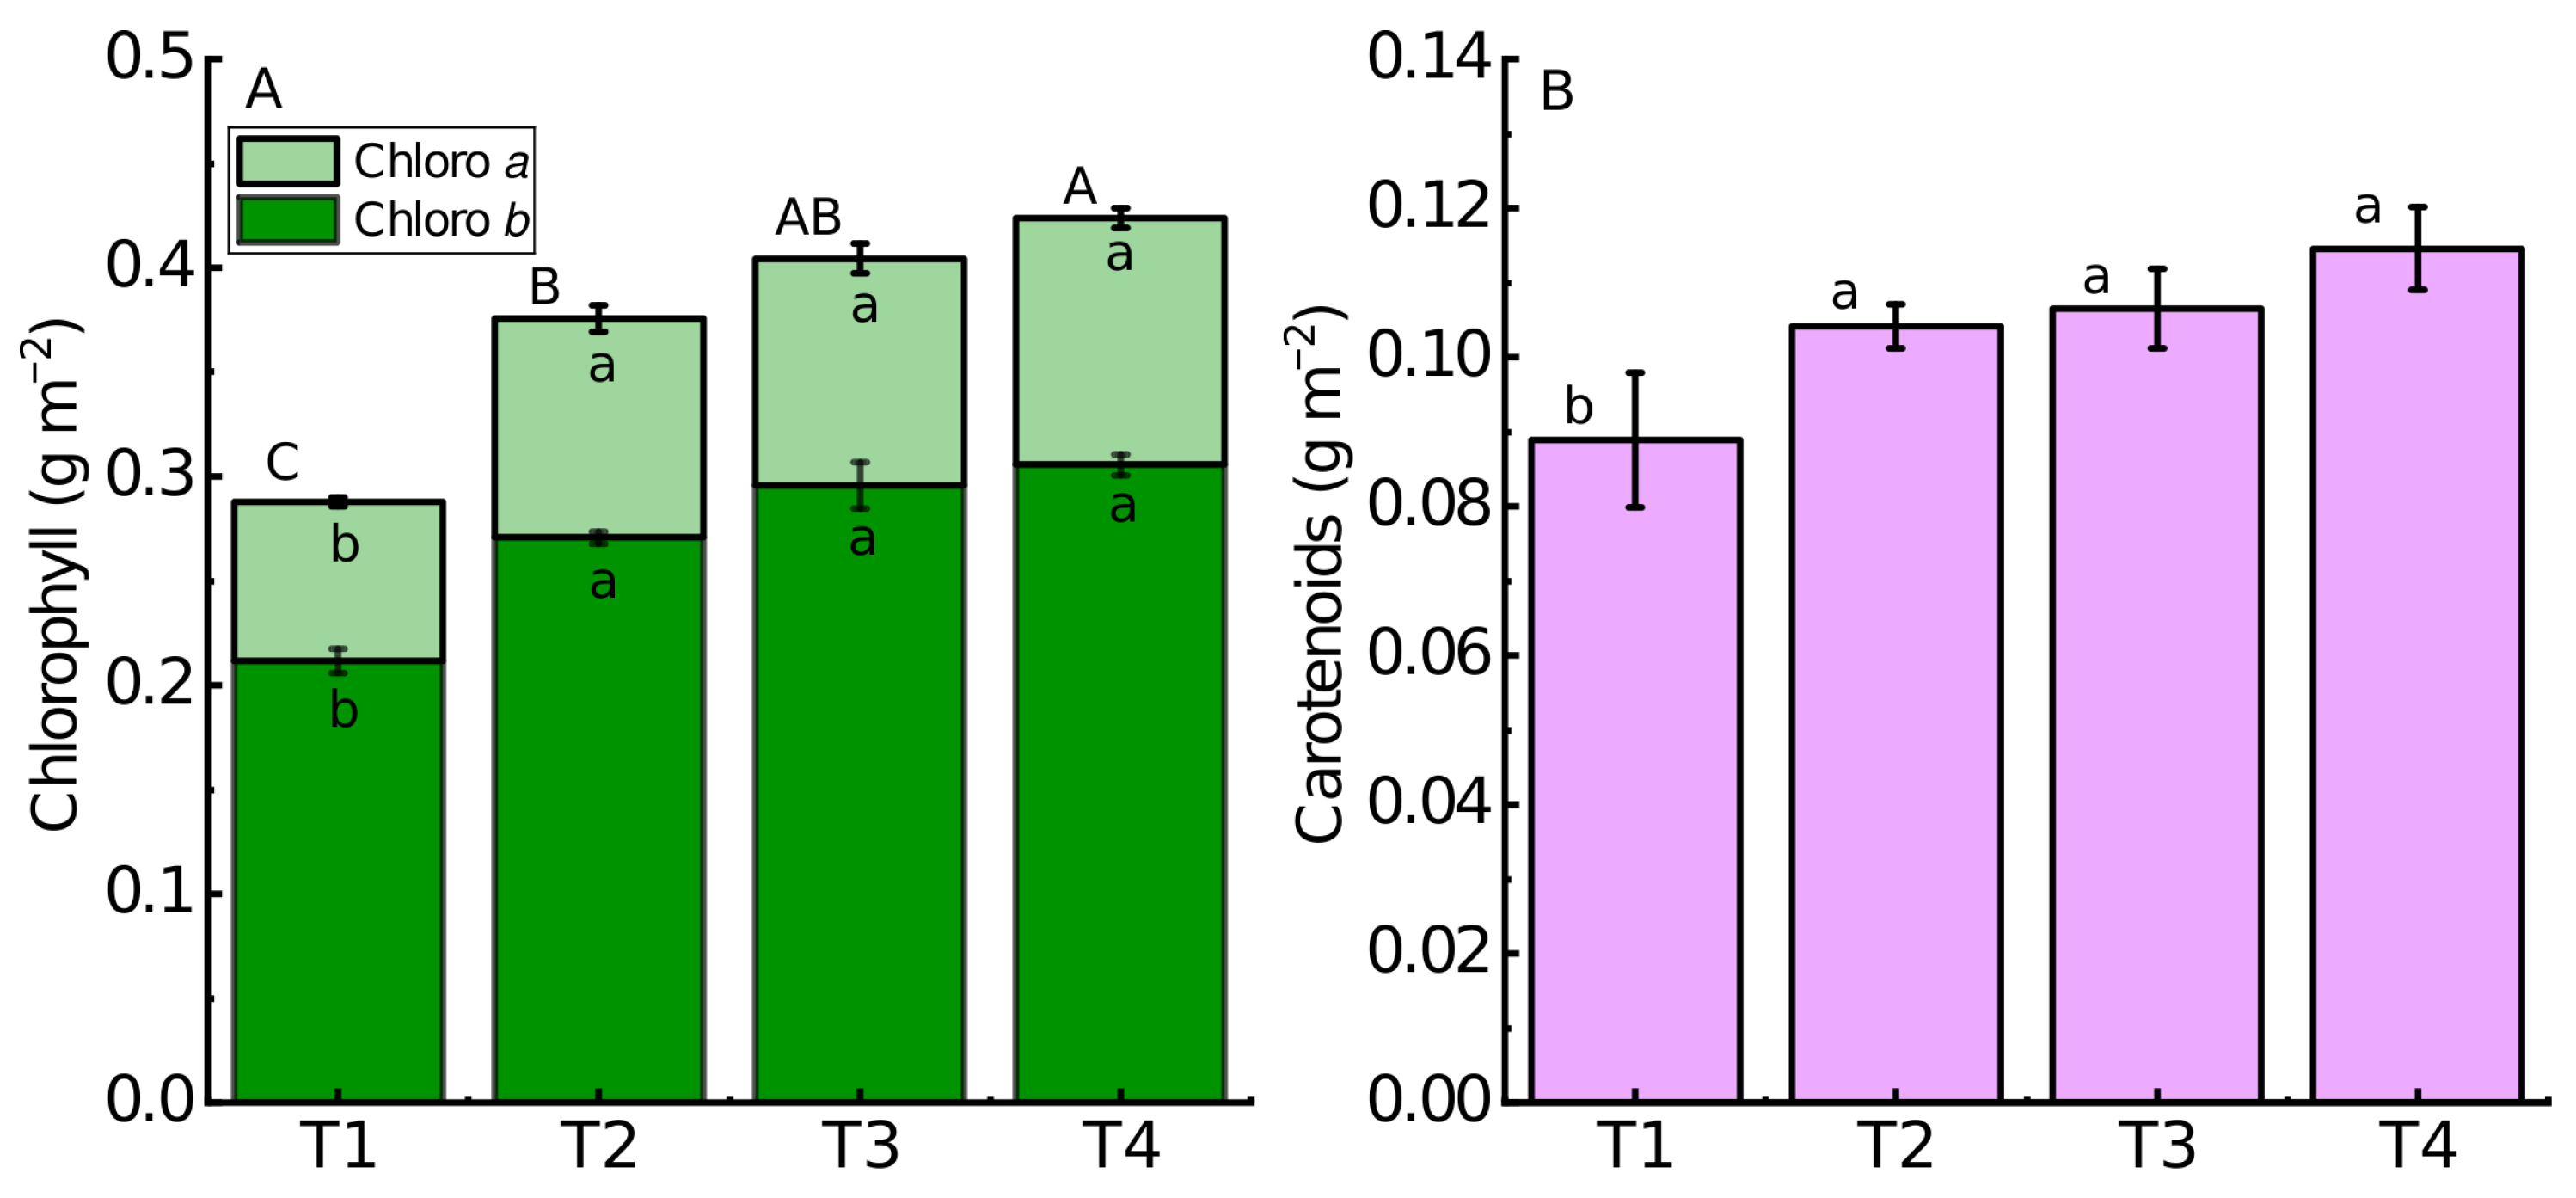
Chlorophyll, a key pigment for light harvesting in photosynthesis, responded positively to biosolid application (Figure 2A). The addition of biosolid alone increased the contents of both chlorophyll a and b, indicating improved photosynthetic pigment synthesis. In contrast, the combined application of biosolid with B. aryabhattai inoculation did not significantly alter the individual chlorophyll fractions. Nevertheless, total chlorophyll content increased in response to biosolid, and this effect was further enhanced when biosolid was combined with B. aryabhattai at 6.4 mL. Although chlorophyll a and chlorophyll b did not differ significantly when analyzed separately, both pigments showed a similar tendency to increase in the inoculated treatments. When combined, these cumulative variations resulted in higher total chlorophyll content. This response suggests a general increase in pigment concentration without major alterations in the relative proportions of chlorophyll a and b, indicating that the overall structure of the photosynthetic apparatus was maintained. Such changes may be associated with improved nutritional status, particularly nitrogen availability, which plays a key role in chlorophyll synthesis and the formation of photosynthetic proteins. This increase in chlorophyll content may be associated with enhanced leaf nutrient availability, particularly N, which is a structural component of the chlorophyll molecule. Although Cu, Mn, and Zn are not structural constituents of chlorophyll, these micronutrients play important regulatory roles in chlorophyll biosynthesis, photosynthetic enzyme activation, and pigment stability [43,44,45]. Consistent with our findings, increases in chlorophyll content following inoculation with B. aryabhattai strains have also been reported under different experimental conditions [17,46,47]. As reported in the literature, presence of B. aryabhattai may have stimulated the production of growth regulators such as cytokinins and indole-3-acetic acid (IAA) or butanoic acid, which help maintain chloroplast integrity and delay chlorophyll degradation [8,17,48].
Sun et al. [49] provide a comprehensive overview of recent advances in carotenoid research in plants, highlighting their multifunctional roles in photosynthesis as accessory light-harvesting pigments and key photoprotective molecules involved in energy dissipation. Carotenoid content increased exclusively in response to biosolid application, suggesting that this effect is primarily driven by improved nutrient supply rather than by B. inoculation (Figure 2B). This response may reflect greater availability of key nutrients involved in carotenoid biosynthesis, contributing to improved protection of the photosynthetic apparatus under the experimental conditions. Azeem et al. [46] also found increase in carotenoids by inoculation with B. aryabhattai strain PM34.

3.4. Growth and Dry Matter Production

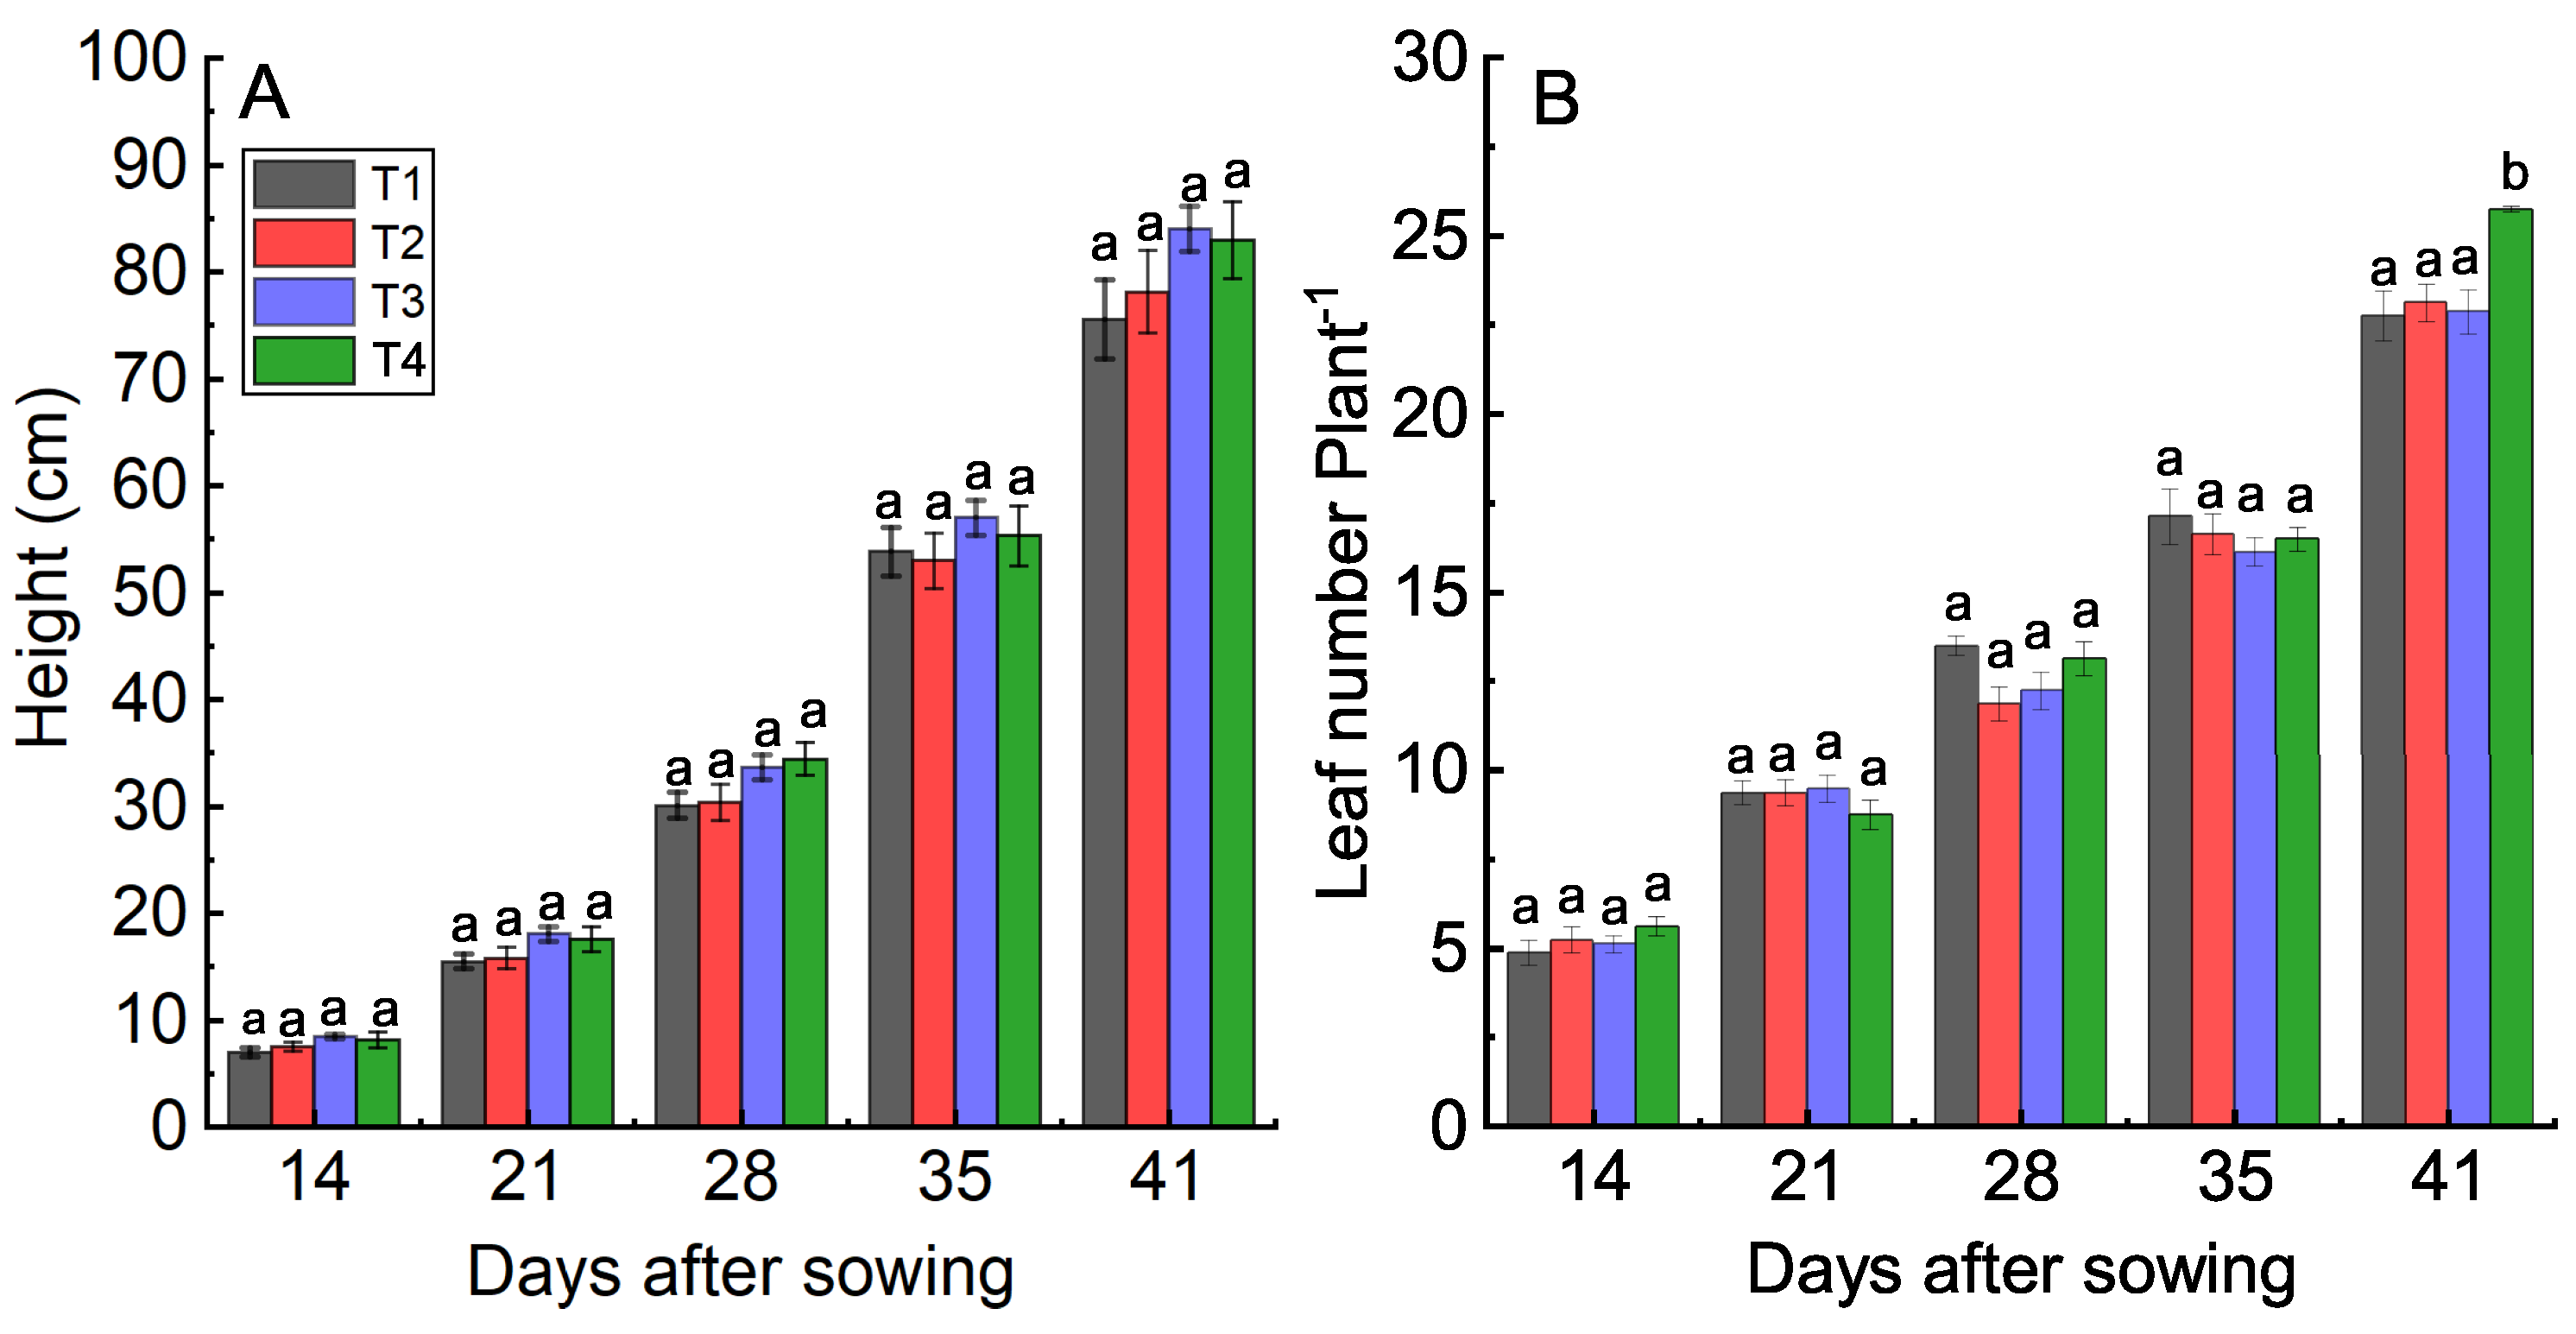
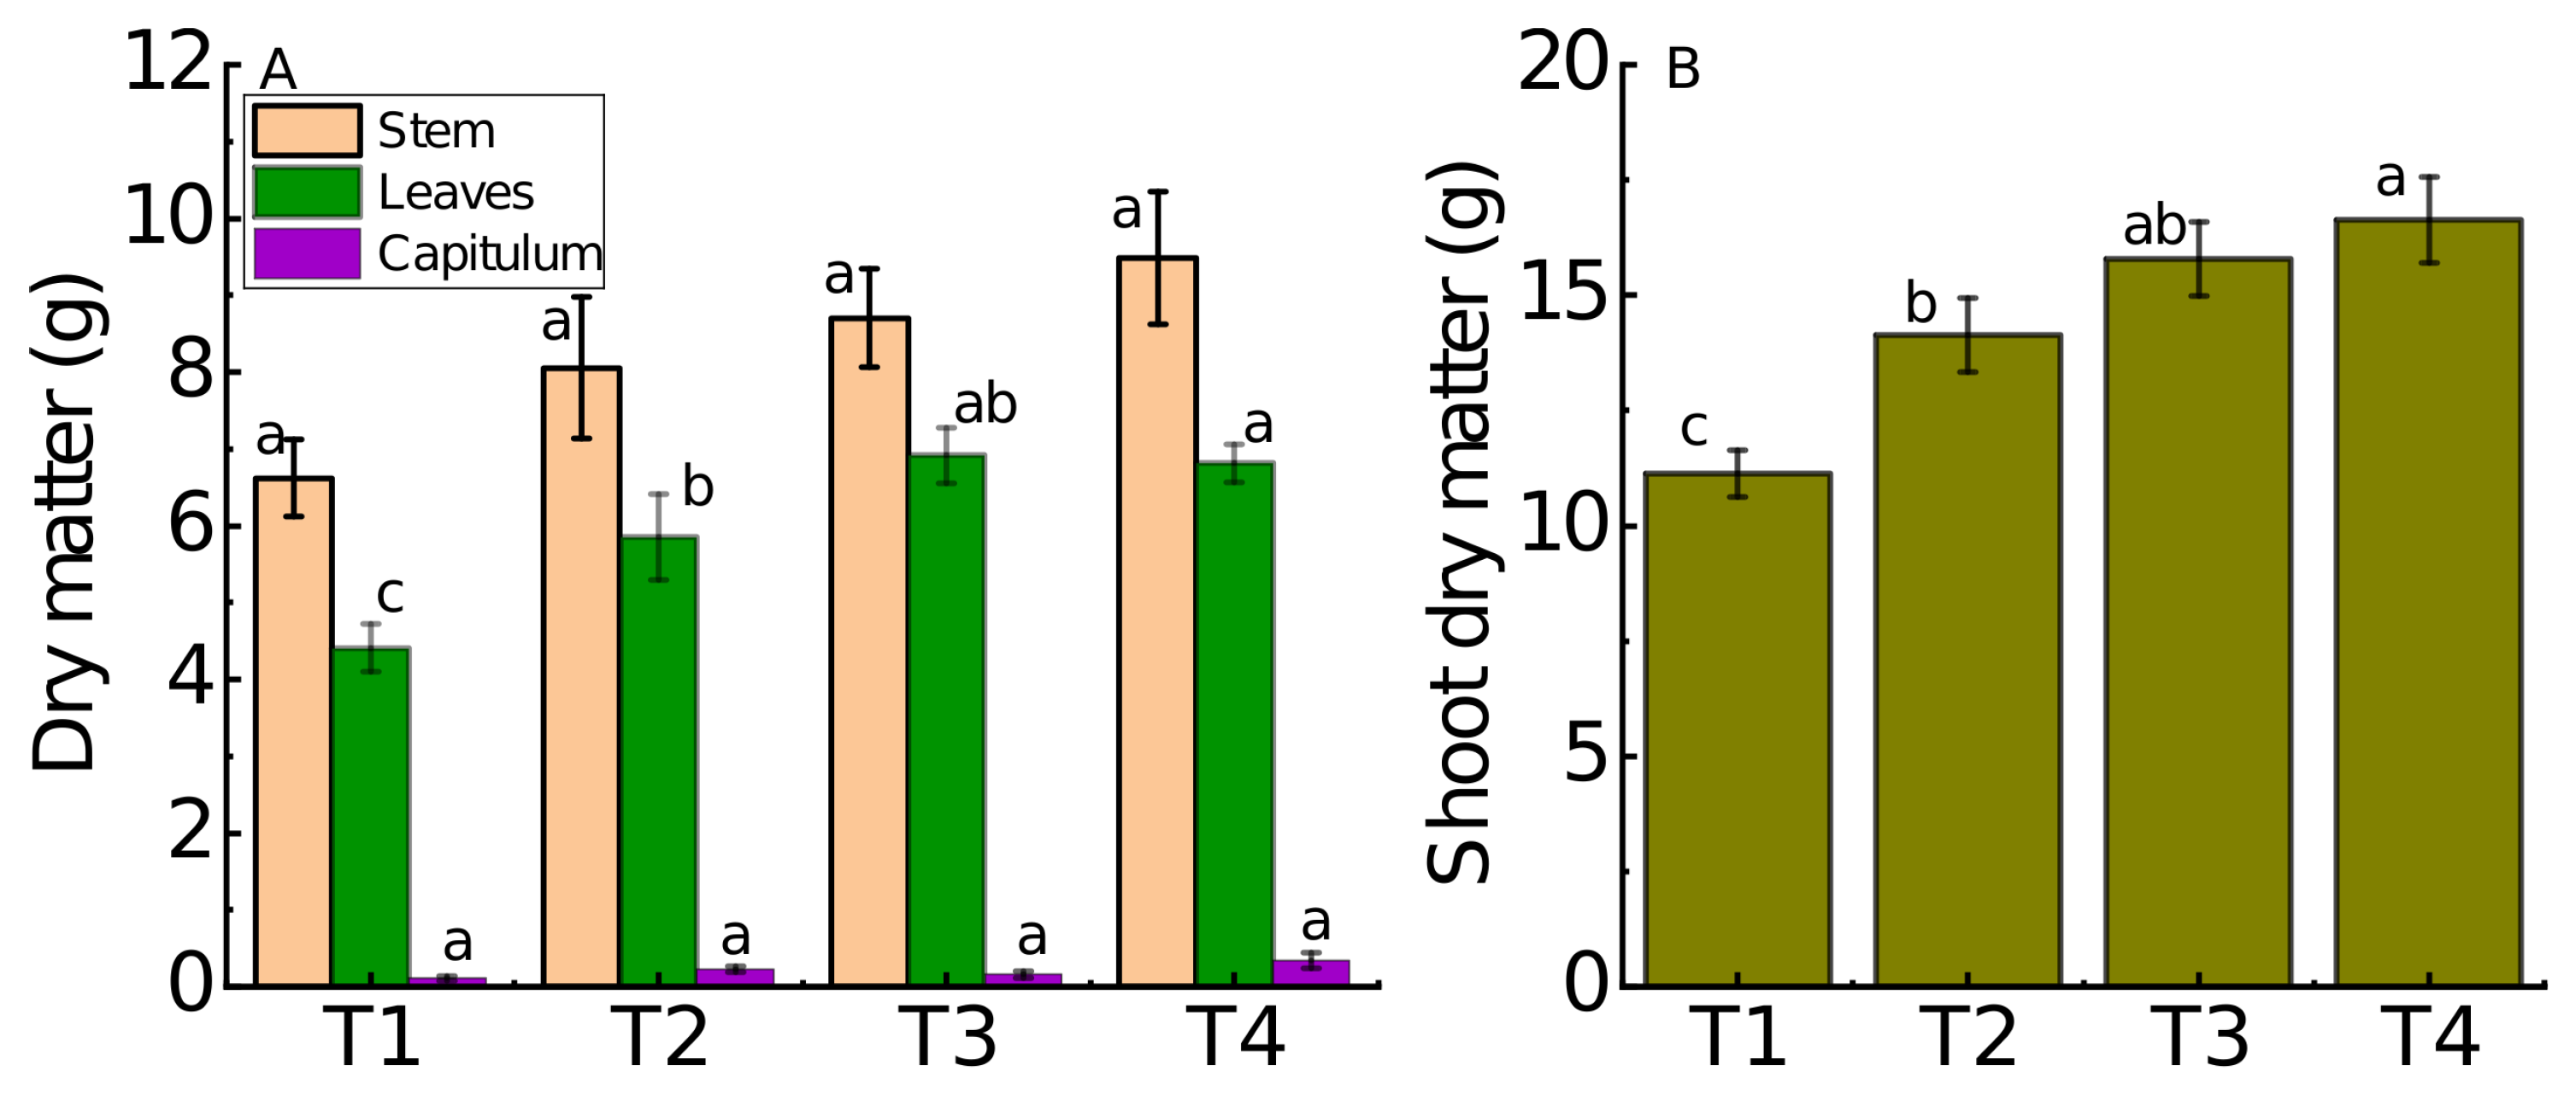
Figure 3A shows that neither the application of biosolid alone nor its combination with B. aryabhatta resulted in an increase in plant height during the growth period. Likewise, no significant difference in leaf number per plant was observed with biosolid application compared to the control treatment (Figure 3B). However, the combined application of biosolid and 6.4 mL of B. aryabhattai led to a higher leaf number per plant at the end of the experimental period compared to the other treatments. Interestingly, although leaf number was not increased by biosolid alone or by its combination with the lower dose of B. aryabhattai, leaf dry matter was significantly higher than in the control plants (Figure 4).
The plant height and leaf number were only slightly affected by the treatments. However, a significant increase in leaf dry mass was observed. This suggests that the treatments primarily promoted biomass accumulation in existing leaves rather than increasing the number of leaves or plant height, possibly through enhanced photosynthetic performance and greater accumulation of photoassimilates. Although no statistically significant difference was detected between the two inoculum doses, the treatment receiving the higher dose tended to show greater responses toward the end of the experimental period.
The results of this study underscore the agronomic potential of biosolids as a sustainable nutrient source for plant development, as evidenced by enhanced vegetative growth and greater dry matter accumulation relative to the control treatment (Figure 4). The additional increase in biomass under the higher dose of B. aryabhattai suggests that bacterial inoculation may enhance plant responses to biosolid application. Plant growth-promoting rhizobacteria are known to improve nutrient availability and uptake through mechanisms such as nutrient solubilization and rhizosphere modification [9,16,32]. These findings align with those of Lucia et al. [50], who highlight that properly treated sewage sludge can be effectively valorized as an agricultural input, contributing to nutrient recycling and soil quality improvement within a circular economy framework. Furthermore, the combined application of biosolids and B. aryabhattai was associated with higher shoot biomass production compared with the biosolid-only treatment (Figure 4). These findings suggest that biosolid and B. aryabhattai can act as complementary bioinputs, contributing to improved plant performance when applied together. Although in the present study the colonization was not directly assessed, scanning electron microscopy conducted by Mun et al. [17] showed that B. aryabhattai SRB02 rapidly and successfully colonizes soybean roots (within 2 days) and exhibits strong potential to promote plant growth through phytohormone production, enhancing nutrient accumulation and chlorophyll stability. The association between PGPR and plant roots enhances nutrients acquisition, photosynthetic performance, and source–sink balance, thereby creating physiological conditions favorable for sustained growth [51]. In particular, B. aryabhattai has been shown to stimulate root development and biomass accumulation [17,47], partly through a ROS-mediated feedback mechanism that promotes bacterial IAA production and root growth [52]. Improved root architecture likely increases nutrient uptake, especially N, which is directly linked to chlorophyll synthesis and Rubisco content, ultimately supporting higher carboxylation efficiency. Moreover, the combined use of bacterial inoculants and sludge has been reported to progressively enhance soil biochemical properties and nutrient availability [22], reinforcing the physiological basis for the higher chlorophyll content, leaf N concentration, and photosynthetic performance observed in the present study under biosolid and B. aryabhattai treatments. Esperschütz et al. [53] demonstrated that agricultural management strategies that enhance microbial biomass and community structure contribute to greater biological activity and soil quality. Similarly, while biosolid improved nutrient supply and plant performance in our study, the inoculation with B. aryabhattai intensified these effects, indicating that biologically driven strategies can further optimize nutrient use efficiency and crop productivity. These findings suggest that microbial inoculation may enhance plant performance during early growth stages, indicating potential for the combined use of biosolids and beneficial microorganisms in sustainable crop management.
It is important to consider that the commercial inoculant used in this study contains not only B. aryabhattai strain CMAA 1363 but also humic substances and other formulation components. Humic substances are known to influence plant growth by stimulating root development, enhancing nutrient availability, and improving nutrient uptake efficiency. Therefore, although the responses observed in the present study are consistent with the plant growth–promoting activities reported for B. aryabhattai, part of the observed effects may also be associated with the presence of humic substances in the formulation. In this sense, the results likely reflect the combined action of the bacterial strain and the other compounds present in the commercial product, which together may contribute to improved plant performance. Although plant responses observed in this study are consistent with the plant growth–promoting activity reported for Bacillus species, the colonization of the rhizosphere by B. aryabhattai was not directly evaluated. Future studies addressing bacterial establishment in the rhizosphere would help to better elucidate the mechanisms responsible for the observed effects. It is important to acknowledge a limitation of the experimental design. The absence of a treatment including B. aryabhattai without biosolid application prevents a clear assessment of the individual effect of the bacterial inoculant. Nevertheless, previous studies have demonstrated that B. aryabhattai alone can significantly improve plant performance under different conditions. For example, Deng et al. [54] showed that B. aryabhattai promotes maize growth by modifying the rhizosphere microbial community. Similarly, Oliveira et al. [55] reported improved agronomic performance and water use efficiency in common bean under deficit irrigation, while Mota et al. [56] demonstrated that B. aryabhattai modulates soil biological activity and enhances plant development under water deficit conditions. These findings support the well-established role of B. aryabhattai as a plant growth-promoting bacterium and reinforce the interpretation that part of the responses observed in the present study may be associated with its biological activity, even though its isolated effect was not directly evaluated. Consequently, the responses observed under combined application should be interpreted with caution, as they may reflect the combined influence of biosolid-derived nutrient supply and bacterial activity rather than the isolated effect of B. aryabhattai. Future studies including treatments with bacterial inoculation alone are needed to better disentangle these effects and quantify the specific contribution of the microorganism. In addition, as the present study focused on short-term plant responses under greenhouse conditions, the long-term application of biosolids in agricultural systems requires careful monitoring, particularly regarding the potential accumulation of nutrients and toxic substances in the soil.

4. Conclusions

In this greenhouse study, the application of sewage sludge–derived biosolid improved plant growth and physiological performance in sunflower during the early growth stage. The addition of B. aryabhattai to biosolid application was associated with further increases in shoot biomass and changes in leaf nutrient composition, suggesting that bacterial inoculation may enhance plant responses under these conditions. However, the absence of a treatment with B. aryabhattai applied without biosolid represents a limitation of the present study, as it restricts the assessment of the isolated effect of the bacterial inoculant. Although the experiment did not evaluate the full crop cycle, the results suggest that the combined use of biosolid and beneficial microorganisms may represent a promising strategy for improving plant performance during early development. Further studies under field conditions and throughout the complete crop cycle are needed to confirm the broader agronomic implications of these findings and to assess the potential accumulation of potential toxic elements or pathogen in the soil following long-term biosolid application.

Author Contributions

Conceptualization, I.C.; data curation, I.C. and L.G.S.; formal analyzes, I.C. and L.G.S.; supervision, I.C.; writing, I.C. and L.G.S.; investigation, I.C., L.G.S., E.F.d.A.S. and A.C.P.; methodology, I.C., L.G.S., E.F.d.A.S. and A.C.P.; writing—review and editing, I.C., L.G.S. and E.F.d.A.S. All authors have read and agreed to the published version of the manuscript.

Funding

This research received no external funding and was conducted using institutional resources.

Data Availability Statement

The study’s original contributions are provided within the article. For additional information, please contact the corresponding author.

Acknowledgments

We thank the São Paulo State Basic Sanitation Company (SABESP) for kindly providing the biosolid (Sabesfertil), and the Rectorate of São Paulo State University for supporting this research.

Conflicts of Interest

The authors declare no conflicts of interest.

References

  1. Xu, J.; Li, Y.; Li, L. A comprehensive review of the effects of organic amendments on soil health and fertility: Mechanisms, greenhouse gas emissions, and implications for sustainable agriculture. Agronomy 2025, 15, 2705. [Google Scholar] [CrossRef] [Scilit]
  2. Hassan, M.K.; Pesonen, J.; Mohsin, M.; Villa, A.; Tuomikoski, S.; Pappinen, A.; Kuittinen, S. Characterization of sewage sludge-based organomineral fertilizers and evaluation of their effectiveness on growth and productivity of spring barley (Hordeum vulgare L.). J. Mater. Cycles Waste Manag. 2025, 27, 2959–2971. [Google Scholar] [CrossRef] [Scilit]
  3. Hu, Y.; Shan, Y. Effects of Sewage Sludge on Soil Physical, Chemical and Biological Properties. Front. Sustain. Dev. 2025, 5, 25–30. [Google Scholar] [CrossRef] [Scilit]
  4. AL-Huqail, A.A.; Kumar, P.; Ahmed, M.T.; Eid, E.M. Cultivation of Turnip Plant (Brassica rapa var. rapa L.) Under Sewage Sludge Amendment: A Lab-Scale Experimental Study. J. Soil Sci. Plant Nutr. 2025, 25, 5607–5625. [Google Scholar] [CrossRef] [Scilit]
  5. Ahmed, M.T.; Alrumman, S.A.; Kumar, P.; Sewelam, N.; Eid, E.M. Growth Response and Heavy Metal Accumulation in Red Radish (Raphanus sativus L.) Under Sewage Sludge Amendment. J. Soil Sci. Plant Nutr. 2025, 26, 642–657. [Google Scholar] [CrossRef] [Scilit]
  6. Dias, S.S.H.; Cubas, A.L.V.; Soares, C.R.F.S.; Giachini, A.J. Sewage sludge in the production of chrysanthemum (Dendranthema grandiflora) and petunia (petunia x hybrida) seedlings. Acta Sci. Agron. 2026, 48, e73355. [Google Scholar] [CrossRef] [Scilit]
  7. Vessey, J.K. Plant growth promoting rhizobacteria as biofertilizers. Plant Soil 2003, 255, 571–586. [Google Scholar] [CrossRef] [Scilit]
  8. Park, Y.G.; Mun, B.G.; Kang, S.M.; Hussain, A.; Shahzad, R.; Seo, C.W.; Kim, A.Y.; Lee, S.U.; Oh, K.Y.; Lee, D.Y.; et al. Bacillus aryabhattai SRB02 tolerates oxidative and nitrosative stress and promotes the growth of soybean by modulating the production of phytohormones. PLoS ONE 2017, 12, e0173203. [Google Scholar] [CrossRef] [Scilit]
  9. Ramesh, A.; Sharma, S.K.; Sharma, M.P.; Yadav, N.; Joshi, O.P. Inoculation of zinc solubilizing Bacillus aryabhattai strains for improved growth, mobilization and biofortification of zinc in soybean and wheat cultivated in Vertisols of central India. Appl. Soil Ecol. 2014, 73, 87–96. [Google Scholar] [CrossRef] [Scilit]
  10. Ahmad, M.; Adil, Z.; Hussain, A.; Mumtaz, M.Z.; Nafees, M.; Ahmad, I.; Jamil, M. Potential of phosphate solubilizing Bacillus strains for improving growth and nutrient uptake in mungbean and maize crops. Pak. J. Agric. Sci. 2019, 56, 283–289. [Google Scholar]
  11. Logan, N.A.; Vos, P.D. Bacillus . In Bergey’s Manual of Systematics of Archaea and Bacteria; Wiley Online Library: Hoboken, NJ, USA, 2015; pp. 1–163. [Google Scholar]
  12. Kavamura, V.N.; Santos, S.N.; da Silva, J.L.; Parma, M.M.; Ávila, L.A.; Visconti, A.; Zucchi, T.D.; Taketani, R.G.; Andreote, F.D.; de Melo, I.S. Screening of Brazilian cacti rhizobacteria for plant growth promotion under drought. Microbiol. Res. 2013, 168, 183–191. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  13. Castelo Sousa, H.; Gomes de Sousa, G.; de Araújo Viana, T.V.; Prudêncio de Araújo Pereira, A.; Nojosa Lessa, C.I.; Pires de Souza, M.V.; da Silva Guilherme, J.M.; Ferreira Goes, G.; da Silveira Alves, F.G.; Primola Gomes, S.; et al. Bacillus aryabhattai mitigates the effects of salt and water stress on the agronomic performance of maize under an agroecological system. Agriculture 2023, 13, 1150. [Google Scholar] [CrossRef] [Scilit]
  14. Farias, M.H.F.; de Melo, A.R.P.; de Freitas, E.M.; Lima, M.A.B.; da Silveira, F.A.; Ferreira, É.G. Biotechnological potential of growth-promoting bacteria in cotton (Gossypium hirsutum L.) crop. Rev. Bras. Ciências Ambient. 2024, 59, e1906. [Google Scholar] [CrossRef] [Scilit]
  15. Siddika, A.; Rashid, A.A.; Khan, S.N.; Khatun, A.; Karim, M.M.; Prasad, P.V.; Hasanuzzaman, M. Harnessing plant growth-promoting rhizobacteria, Bacillus subtilis and B. aryabhattai to combat salt stress in rice: A study on the regulation of antioxidant defense, ion homeostasis, and photosynthetic parameters. Front. Plant Sci. 2024, 15, 1419764. [Google Scholar] [CrossRef] [Scilit]
  16. Rafique, E.; Mumtaz, M.Z.; Li, L.; Ullah, I.; Chohan, T.A.; Alam, M.W.; Mustafa, A.; Alsakkaf, W.A.; Ali, H.M. Plant Growth Promoting Rhizobacteria Regulated Nutrient Uptake in Quinoa (Chenopodium quinoa Wild) Under Nutrient-Deficient Conditions Through Solubilizing Insoluble Minerals. J. Soil Sci. Plant Nutr. 2025, 25, 4629–4652. [Google Scholar] [CrossRef] [Scilit]
  17. Mun, B.G.; Hussain, A.; Park, Y.G.; Kang, S.M.; Lee, I.J.; Yun, B.W. The PGPR Bacillus aryabhattai promotes soybean growth via nutrient and chlorophyll maintenance and the production of butanoic acid. Front. Plant Sci. 2024, 15, 1341993. [Google Scholar] [CrossRef] [Scilit]
  18. Fuga, C.A.G.; Caixeta, G.A.N.; Caixeta, C.F.; de Melo, I.S. Growth promotion in maize (Zea mays L.) by Bacillus aryabhattai strain CMAA 1363. Rev. Bras. Ciências Agrárias 2023, 18, e3340. [Google Scholar]
  19. May, A.; Ramos, N.P.; dos Santos, M.d.S.; da Silva, E.H.F.M.; de Melo, I.S. Promoção de Crescimento de Mudas Pré-Brotadas de Cana-de-Açúcar Inoculadas com Bacillus aryabhattai em Diferentes Frequências de Irrigação. 2019. Available online: https://www.infoteca.cnptia.embrapa.br/infoteca/bitstream/doc/1107857/1/boletim80Andre.pdf (accessed on 7 April 2026).
  20. Van Chuong, N.; Tri, T.L.K.; Vu, T.M.; Tuan, L.M.; Liem, T.T.; Trang, N.N.P. Isolation and identification of Bacillus aryabhattai M2C: Its effects with vermicompost on yield and nutrients of peanut (Arachis hypogaea L.). Int. J. Microbiol. 2025, 2025, 9923279. [Google Scholar] [CrossRef] [Scilit]
  21. Hasan, M.; Naushin, F.; Shaher, H.; Bagyaraj, D. Influence of sewage sludge, Rhizobium and arbuscular mycorrhizal fungi on nutrient uptake, growth, photosynthetic and biochemical attributes in Cicer arietinum L. Braz. J. Bot. 2023, 46, 1161–1176. [Google Scholar] [CrossRef] [Scilit]
  22. Ren, H.; Chen, X.; Qin, X.; Zhang, S.; Lv, C.; Zhou, J.; Chen, H. Bacterial fertilizer and filtered sludge enhance soil fertility and plant growth in a eucalyptus plantation. Silva Fenn. 2024, 58, 24042. [Google Scholar] [CrossRef] [Scilit]
  23. Rondon, O.H.S.; de Faria, D.A.; Avelino, A.C.D.; Pallaoro, D.S.; Filho, A.B.B.; de Matos, V.A.T.; de Abreu, J.G.; Nadin, W.; Peixoto, W.M.; e Silva, Y.R.V.B.; et al. Agronomic Characteristics Correlation of Sunflower Genotypes Grown in the Second Crop in the Cerrado. J. Exp. Agric. Int. 2019, 36, 1–9. [Google Scholar] [CrossRef] [Scilit]
  24. Lichtenthaler, H.K. [34] Chlorophylls and carotenoids: Pigments of photosynthetic biomembranes. In Methods in Enzymology; Elsevier: Amsterdam, The Netherlands, 1987; Volume 148, pp. 350–382. [Google Scholar]
  25. MAPA. Manual de Métodos Analíticos Oficiais para Fertilizantes e Corretivos/Ministério da Agricultura, Pecuária e Abastecimento, 2017. Available online: https://www.gov.br/agricultura/pt-br/assuntos/insumos-agropecuarios/insumos-agricolas/fertilizantes/legislacao/manual-de-metodos_2017_isbn-978-85-7991-109-5.pdf (accessed on 7 April 2026).
  26. Antonkiewicz, J.; Baran, A.; Kopta, T.; Lošák, T.; Ryant, P. From biowaste to fertiliser. In The Circular Bioeconomy; Routledge: London, UK, 2025; p. 322. [Google Scholar]
  27. Bettiol, W.; Camargo, O. Lodo de Esgoto: Impactos Ambientais na Agricultura; Embrapa Meio Ambiente: Jaguariúna, Brazil, 2006; Available online: https://www.researchgate.net/profile/Carolina-Leoni/publication/265028920_Efeito_do_lodo_de_esgoto_na_inducao_de_supressividade_de_solos_a_Phytophthora_nicotianae_em_citros/links/53fc83f00cf2dca8ffff2a44/Efeito-do-lodo-de-esgoto-na-inducao-de-supressividade-de-solos-a-Phytophthora-nicotianae-em-citros.pdf (accessed on 7 April 2026).
  28. Fytili, D.; Zabaniotou, A. Utilization of sewage sludge in EU application of old and new methods—A review. Renew. Sustain. Energy Rev. 2008, 12, 116–140. [Google Scholar] [CrossRef] [Scilit]
  29. Garg, N.; Singh, S. Arbuscular mycorrhiza Rhizophagus irregularis and silicon modulate growth, proline biosynthesis and yield in Cajanus cajan L. Millsp. (pigeonpea) genotypes under cadmium and zinc stress. J. Plant Growth Regul. 2018, 37, 46–63. [Google Scholar] [CrossRef] [Scilit]
  30. Brazil. Resolução №498, de 19 de agosto de 2020. Define critérios e procedimentos para produção e aplicação de biossólido em solos, e dá outras providências. Diário Of. República Fed. Bras. 2020, 161, 265. [Google Scholar]
  31. Quaggio, J.; Alcântara, P.; Cantarella, H.; Paulino, V.; Villa, M. BOLETIM 100: Recomendação de Adubação e Calagem para o Estado de São Paulo; IAC Campinas: Campinas, Brazil, 2022. [Google Scholar]
  32. Srithaworn, M.; Jaroenthanyakorn, J.; Tangjitjaroenkun, J.; Suriyachadkun, C.; Chunhachart, O. Zinc solubilizing bacteria and their potential as bioinoculant for growth promotion of green soybean (Glycine max L. Merr.). PeerJ 2023, 11, e15128. [Google Scholar] [CrossRef] [Scilit]
  33. Pérez-Novo, C.; Bermúdez-Couso, A.; López-Periago, E.; Fernández-Calviño, D.; Arias-Estévez, M. Zinc adsorption in acid soils: Influence of phosphate. Geoderma 2011, 162, 358–364. [Google Scholar] [CrossRef] [Scilit]
  34. Antolín, M.C.; Muro, I.; Sánchez-Díaz, M. Application of sewage sludge improves growth, photosynthesis and antioxidant activities of nodulated alfalfa plants under drought conditions. Environ. Exp. Bot. 2010, 68, 75–82. [Google Scholar] [CrossRef] [Scilit]
  35. Farquhar, G.D.; von Caemmerer, S.V.; Berry, J.A. A biochemical model of photosynthetic CO2 assimilation in leaves of C3 species. Planta 1980, 149, 78–90. [Google Scholar] [CrossRef] [Scilit]
  36. Flexas, J.; Medrano, H. Drought-inhibition of photosynthesis in C3 plants: Stomatal and non-stomatal limitations revisited. Ann. Bot. 2002, 89, 183–189. [Google Scholar] [CrossRef] [Scilit]
  37. Flexas, J.; Ribas-Carbo, M.; Diaz-Espejo, A.; Galmés, J.; Medrano, H. Mesophyll conductance to CO2: Current knowledge and future prospects. Plant Cell Environ. 2008, 31, 602–621. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  38. Monalisa, S.; Roy, S. Chapter-5 Effect of Biopriming with Plant Growth Promoting Rhizobacteria (PGPR). In Research Trends in Agriculture Sciences; Naresh, R.K., Ed.; AkiNik Publications: New Delhi, India, 2022; p. 73. [Google Scholar]
  39. Kitajima, K.; Mulkey, S.S.; Samaniego, M.; Wright, S.J. Decline of photosynthetic capacity with leaf age and position in two tropical pioneer tree species. Am. J. Bot. 2002, 89, 1925–1932. [Google Scholar] [CrossRef] [Scilit]
  40. Zhou, W.; Ling, J.; Shen, X.; Xu, Z.; Yang, Q.; Yue, W.; Liu, H.; Suo, A.; Dong, J. Inoculation with plant growth-promoting rhizobacteria improves seagrass Thalassia hemprichii photosynthesis performance and shifts rhizosphere microbiome. Mar. Environ. Res. 2024, 193, 106260. [Google Scholar] [CrossRef] [Scilit]
  41. Egamberdieva, D.; Wirth, S.J.; Alqarawi, A.A.; Abd_Allah, E.F.; Hashem, A. Phytohormones and beneficial microbes: Essential components for plants to balance stress and fitness. Front. Microbiol. 2017, 8, 2104. [Google Scholar] [CrossRef] [Scilit]
  42. Lee, S.; Ka, J.O.; Song, H.G. Growth promotion of Xanthium italicum by application of rhizobacterial isolates of Bacillus aryabhattai in microcosm soil. J. Microbiol. 2012, 50, 45–49. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  43. Cakmak, I. Tansley Review No. 111 Possible roles of zinc in protecting plant cells from damage by reactive oxygen species. New Phytol. 2000, 146, 185–205. [Google Scholar] [CrossRef] [Scilit]
  44. Millaleo, R.; Reyes-Díaz, M.; Ivanov, A.G.; Mora, M.; Alberdi, M. Manganese as essential and toxic element for plants: Transport, accumulation and resistance mechanisms. J. Soil Sci. Plant Nutr. 2010, 10, 470–481. [Google Scholar] [CrossRef] [Scilit]
  45. Ammara, H.; Zulfiqar, A.; Saleem, A.; Sardar, R.; Zulfiqar, U.; Raza, M.A.S.; Maqsood, M.F.; El-Beltagi, H.S.; Alqahtani, M.D. Zinc-regulated growth, chlorophyll, and antioxidant activity drive biofortification in rice varieties. BioMetals 2026, 39, 375–388. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  46. Azeem, M.A.; Khan, S.; Ali, F.; Ahmad, S.; Rahim, G.; Iftikhar, M.; Iqbal, M.; Aljaloud, R.S.; Alarjani, K.M.; Chaudhary, H.J. Halotolerant Bacillus Aryabhattai strain PM34 mitigates salinity stress and enhances the physiology and growth of maize. J. Plant Growth Regul. 2025, 44, 7000–7018. [Google Scholar] [CrossRef] [Scilit]
  47. Shafqat, A.; Siddiqua, A.; Akram, W.; Kazmi, A.; Altalhi, A.; Akthar, S.; Ambreen, M. Induction of Physiological Resistance Against Fusarium Wilt in Cucumis sativus Using Bacillus aryabhattai Z-48 and Bacillus cereus Z-53. J. Basic Microbiol. 2025, 65, e70121. [Google Scholar] [CrossRef] [Scilit]
  48. Bhattacharyya, C.; Bakshi, U.; Mallick, I.; Mukherji, S.; Bera, B.; Ghosh, A. Genome-guided insights into the plant growth promotion capabilities of the physiologically versatile Bacillus aryabhattai strain AB211. Front. Microbiol. 2017, 8, 411. [Google Scholar] [CrossRef] [Scilit]
  49. Sun, T.; Rao, S.; Zhou, X.; Li, L. Plant carotenoids: Recent advances and future perspectives. Mol. Hortic. 2022, 2, 3. [Google Scholar] [CrossRef] [Scilit]
  50. Lucia, C.; Badalucco, L.; Corsino, S.F.; Galati, A.; Iovino, M.; Muscarella, S.M.; Paliaga, S.; Torregrossa, M.; Laudicina, V.A. Management and valorisation of sewage sludge to foster the circular economy in the agricultural sector. Discov. Soil 2025, 2, 80. [Google Scholar] [CrossRef] [Scilit]
  51. Ilangumaran, G.; Smith, D.L. Plant growth promoting rhizobacteria in amelioration of salinity stress: A systems biology perspective. Front. Plant Sci. 2017, 8, 1768. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  52. Deng, C.; Zeng, N.; Li, C.; Pang, J.; Zhang, N.; Li, B. Mechanisms of ROS-mediated interactions between Bacillus aryabhattai LAD and maize roots to promote plant growth. BMC Microbiol. 2024, 24, 327. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  53. Esperschütz, J.; Gattinger, A.; Mäder, P.; Schloter, M.; Fließbach, A. Response of soil microbial biomass and community structures to conventional and organic farming systems under identical crop rotations. FEMS Microbiol. Ecol. 2007, 61, 26–37. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  54. Deng, C.; Zhang, N.; Liang, X.; Huang, T.; Li, B. Bacillus aryabhattai LAD impacts rhizosphere bacterial community structure and promotes maize plant growth. J. Sci. Food Agric. 2022, 102, 6650–6657. [Google Scholar] [CrossRef] [Scilit]
  55. Oliveira, A.L.; Santos, J.P.; Silva, G.F.; Putti, F.F. Bacillus aryabhattai Improves Agronomic Performance and Water Use Efficiency of Common Bean Under Deficit Irrigation Levels. Crops 2026, 6, 38. [Google Scholar] [CrossRef] [Scilit]
  56. da Silva Mota, K.; Garcia, K.G.V.; de Sousa Almeida, M.; Barbosa, F.L.A.; Borges, W.L.; Mesquita, R.O.; Araujo, A.S.F.; de Sousa, G.G.; de Araujo Pereira, A.P. Bacillus aryabhattai and silicon modulate soil biological activity and performance of Mimosa caesalpiniifolia under water deficit. Braz. J. Microbiol. 2026, 57, 84. [Google Scholar] [CrossRef] [Scilit]
Figure 1. (A) Stomatal conductance (gs), (B) Photosynthesis (A), (C) CO2 concentration in the substomatal cavity (Ci), and (D) Apparent carboxylation efficiency (A/Ci), of sunflower plants grown under biosolid application and Bacillus aryabhattai inoculation. Values are mean ± SE of 10 plants. Significant differences (p < 0.05) among treatments are indicated by different lowercase letters. T1: Substrate + 0 g of biosolid + 0 mL of Bacillus aryabhattai; T2: Substrate + 5 g of biosolid + 0 mL of Bacillus aryabhattai; T3: Substrate + 5 g of biosolid + 3.2 mL of Bacillus aryabhattai; T4: Substrate + 5 g of biosolid + 6.4 mL of Bacillus aryabhattai.
Agronomy 16 00796 g001
Figure 2. (A) Content of chlorophyll a and b and (B) Carotenoids in sunflower plants grown under the biosolid application and Bacillus aryabhattai inoculation. Values are mean ± SE of 5 plants. Significant differences (p < 0.05) among treatments are indicated by different lowercase letters, while significant differences in total chlorophyll content are indicated by uppercase letters. T1: Substrate + 0 g of biosolid + 0 mL of Bacillus aryabhattai; T2: Substrate + 5 g of biosolid + 0 mL of Bacillus aryabhattai; T3: Substrate + 5 g of biosolid + 3.2 mL of Bacillus aryabhattai; T4: Substrate + 5 g of biosolid + 6.4 mL of Bacillus aryabhattai.
Agronomy 16 00796 g002
Figure 3. (A) Plant height and (B) Number of leaves per plant (B) of sunflower grown under biosolid application and Bacillus aryabhattai inoculation. Values are mean ± SE of 8 plants. Significant differences (p < 0.05) among treatments are indicated by different lowercase letters. T1: Substrate + 0 g of biosolid + 0 mL of Bacillus aryabhattai; T2: Substrate + 5 g of biosolid + 0 mL of Bacillus aryabhattai; T3: Substrate + 5 g of biosolid + 3.2 mL of Bacillus aryabhattai; T4: Substrate + 5 g of biosolid + 6.4 mL of Bacillus aryabhattai.
Agronomy 16 00796 g003
Figure 4. (A) Dry mass partitioning of the aerial part and (B) Total shoot dry matter (B) of sunflower plants grown under biosolid application and Bacillus aryabhattai. Values are mean ± SE of 6 plants. Significant differences (p < 0.05) among treatments are indicated by different lowercase letters. T1: Substrate + 0 g of biosolid + 0 mL of Bacillus aryabhattai; T2: Substrate + 5 g of biosolid + 0 mL of Bacillus aryabhattai; T3: Substrate + 5 g of biosolid + 3.2 mL of Bacillus aryabhattai; T4: Substrate + 5 g of biosolid + 6.4 mL of Bacillus aryabhattai.
Agronomy 16 00796 g004
Table 1. Chemical characterization of pure Carolina Soil®.
Macronutrients (g Kg−1)Micronutrients (mg Kg−1)
N P K Ca Mg S B Cu Fe Mn Zn
6.02.82.57.320.12.020.010.032.0184.025.0
Water Retention Capacity (WRC) = 51.0%. pH = 5.1.
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.