Article

Protective Effects of Carvacrol Against Vibrio harveyi Infection in Sebastes schlegelii and Its Underlying Mechanisms


1
National Pathogen Collection Center for Aquatic Animals, Shanghai Engineering Research Center of Aquaculture, National Demonstration Center for Experimental Fisheries Science Education, Shanghai Ocean University, Shanghai 200120, China
2
State Key Laboratory of Mariculture Biobreeding and Sustainable Goods, Yellow Sea Fisheries Research Institute, Chinese Academy of Fishery Sciences, Qingdao 266000, China
3
Laboratory for Marine Fisheries Science and Food Production Processes, Qingdao National Laboratory for Marine Science and Technology, Qingdao 266000, China
4
Huanghua Jinhui Aquaculture Development Co., Ltd., Cangzhou 061000, China
*
Authors to whom correspondence should be addressed.
Fishes 2026, 11(5), 273; https://doi.org/10.3390/fishes11050273
Submission received: 13 March 2026 / Revised: 10 April 2026 / Accepted: 21 April 2026 / Published: 6 May 2026
(This article belongs to the Special Issue Fish Disease Prevention: Immune Defense and Vaccine Development)

Abstract

The inappropriate use of antibiotics in aquaculture has exacerbated antimicrobial resistance in pathogens, thereby reducing the efficiency of aquaculture production. Therefore, it is crucial to develop effective antibiotic alternatives capable of inhibiting pathogenic bacteria. Against this background, the present study investigated the efficacy and underlying mechanism of carvacrol against Vibrio harveyi in the mariculture of the marine fish Sebastes schlegelii, aiming to provide data support for the development of green fishery drugs to replace antibiotics. The results indicated that pre-treatment with carvacrol increased the survival rate of infected S. schlegelii. Meanwhile, post-infection administration of carvacrol alleviated intestinal pathological damage. Carvacrol regulated host immunity by modulating the transcription of the immune-related genes NF-κB/RelA and IL-15. Carvacrol did not significantly alter the activities of SOD, MDA, or CAT, suggesting that the oxidative defense pathway was not primarily involved. Analysis of intestinal Vibrio load confirmed that carvacrol could inhibit the growth and colonization of intestinal Vibrio, thereby maintaining microbial homeostasis. Immunohistochemistry and peripheral blood flow cytometry showed that carvacrol enhanced the adaptive immunity of fish by increasing the proportions of CD4-1+ T cells and CD79a/CD79b+ B cells in tissues and peripheral blood. In conclusion, carvacrol enhances the resistance of S. schlegelii against V. harveyi by inhibiting pathogenic bacteria, improving intestinal morphological structure, reducing pathogenic bacterial load to maintain microbial homeostasis, and enhancing the adaptive immunity of the organism. This study provides a theoretical basis and data support for the substitution of antibiotics and the development of green feed additives in aquaculture.
Key Contribution: This study elucidated the efficacy and mechanism of carvacrol, a CHM monomer, in enhancing the resistance of S. schlegelii against V. harveyi infection and improving the survival rate. Carvacrol is expected to serve as a safe alternative to antibiotics in mariculture, thereby reducing the development of antimicrobial resistance and residues of antimicrobials.

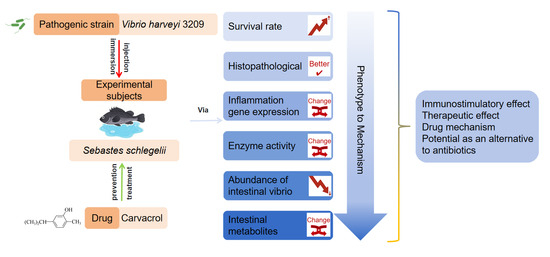
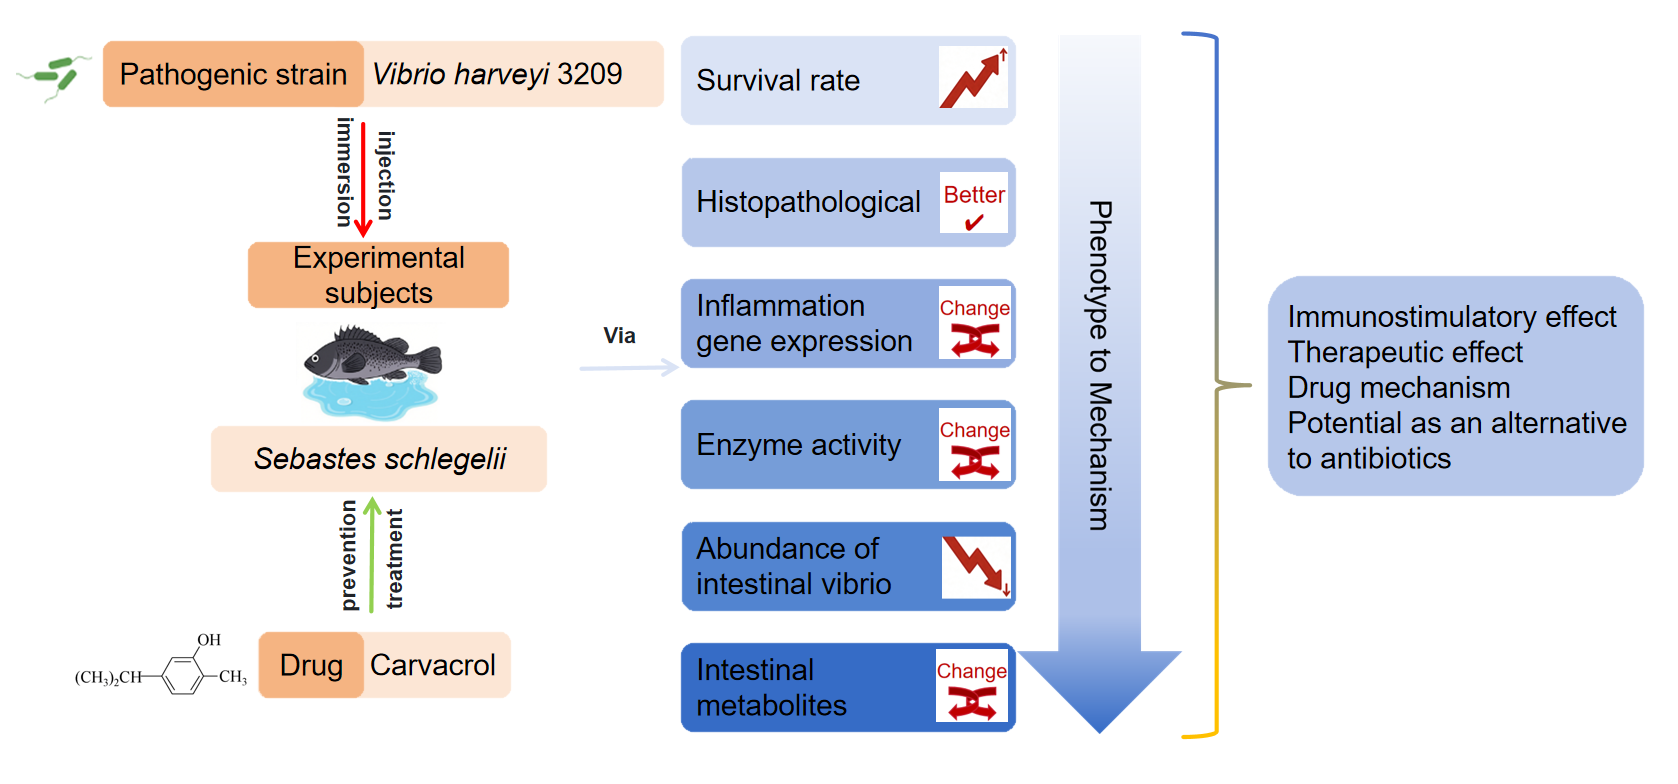
Graphical Abstract

1. Introduction

Aquaculture has emerged as the leading source of global aquatic products supply. Nevertheless, the frequent occurrence of diseases has led to a significant reduction in the yield of certain aquaculture species and a subsequent decline in economic returns. Bacterial diseases represent the predominant category of ailments in aquaculture [1].
Species of Vibrio are among the most harmful pathogens to aquatic animals in the marine environment, causing high mortality rates among aquaculture animals [2,3]. Species such as Vibrio harveyi, Vibrio alginolyticus, and Vibrio vulnificus pose considerable risks to the health of farmed fish [4]. V. harveyi, a Gram-negative marine bacterium, is widely distributed in the environment and affects a variety of marine vertebrates and invertebrates [5]. Fish infected with V. harveyi can display a diverse range of clinical symptoms, including growth retardation, spiral or irregular swimming, dark pigmentation of the skin, the appearance of ulcers and blood clots on the body surface, increased secretion of mucus, eye opacity and lesions, bleeding in the oral area and around internal organs. In acute outbreaks, it can result in the high mortality rate of farmed fish [6,7,8].
Antibiotics serve as one of the primary means for the prevention and treatment of bacterial diseases in aquatic animals. However, the improper utilization of antibiotics in aquaculture promotes drug resistance in pathogenic bacteria, which not only hinders their eradication but also further reduces the profitability of farming. Therefore, it is of great necessity to develop effective antibiotic alternatives that can inhibit pathogenic bacteria [9,10]. Currently, apart from the use of antibiotics, the primary strategies to reduce aquaculture losses caused by these pathogens include researching and developing Chinese herbal medicines, probiotics [11,12], antimicrobial peptides [13,14] and vaccines [15,16]. Chinese Herbal Medicines (CHM) have attracted extensive attention due to their natural origin, low toxicity, and minimal side-effects. Additionally, they can effectively prevent and treat bacterial and viral diseases, enhance immunity, and improve antioxidant capacity [17,18,19]. Nevertheless, traditional CHMs present problems such as complex compositions, poor drug stability, and potential drug interactions [20]. Therefore, it is highly necessary to develop CHM monomers with well-defined drug mechanisms and targeted therapeutic effects. A multitude of studies have demonstrated that Chinese herbal essential oils (EOs) exhibit antimicrobial activity and can enhance the growth performance, immunity, and antioxidant activity of organisms [21,22,23]. Carvacrol is the primary component of essential oils derived from Cinnamomum cassia Presl and Origanum vulgare L. [24]. It exerts an effective inhibitory effect on some pathogenic bacteria in aquaculture, including Vibrio cholerae, Vibrio parahaemolyticus, V. alginolyticus, V. anguillarum, and V. harveyi [25,26,27]. Carvacrol shows similar effects to the mentioned Chinese herbal essential oils in improving growth performance, immunity, and antioxidant activity [28,29].
Studies on the preventive and therapeutic effects of carvacol against Vibrio infections in marine fish, as well as its mechanism of action, are scarce. For this reason, we conducted a series of experiments on juvenile S. schlegelii to systematically evaluate the preventive and immunostimulatory effects of carvacrol, as well as its therapeutic efficacy following infection with V. harveyi. Therefore, in this study, S. schlegelii was selected as the experimental subject. Through a comprehensive analysis of the changes in apparent symptoms, survival rate, intestinal pathological sections, enzyme activity, quantitative expression of inflammatory genes, and pathogenic microbial load after the action of V. harveyi and carvacrol, and by investigating the effects of carvacrol preventive administration on the proportions of changes in CD4-1+ T cells, CD79a+ B cells, and CD79b+ B cells in key immune tissues and peripheral blood, this research systematically explores the preventive and immunity-enhancing effects of carvacrol on juvenile S. schlegelii without pathogenic bacteria infection, as well as its therapeutic effects after pathogenic bacteria infection. Our findings aim to provide a novel antibiotic-alternative strategy for controlling V. harveyi in marine fish farming, while also offering references for the subsequent development of new fishery drugs.

2. Materials and Methods

2.1. Strain

Vibrio harveyi (Strain No. V3209) was originally isolated from diseased S. schlegelii exhibiting characteristic integumentary lesions and maintained at the Yellow Sea Fisheries Research Institute. V. harveyi was cultured in tryptic soy broth (TSB) additionally supplemented with 1% NaCl at 28 °C.

2.2. Fish Management and Sampling

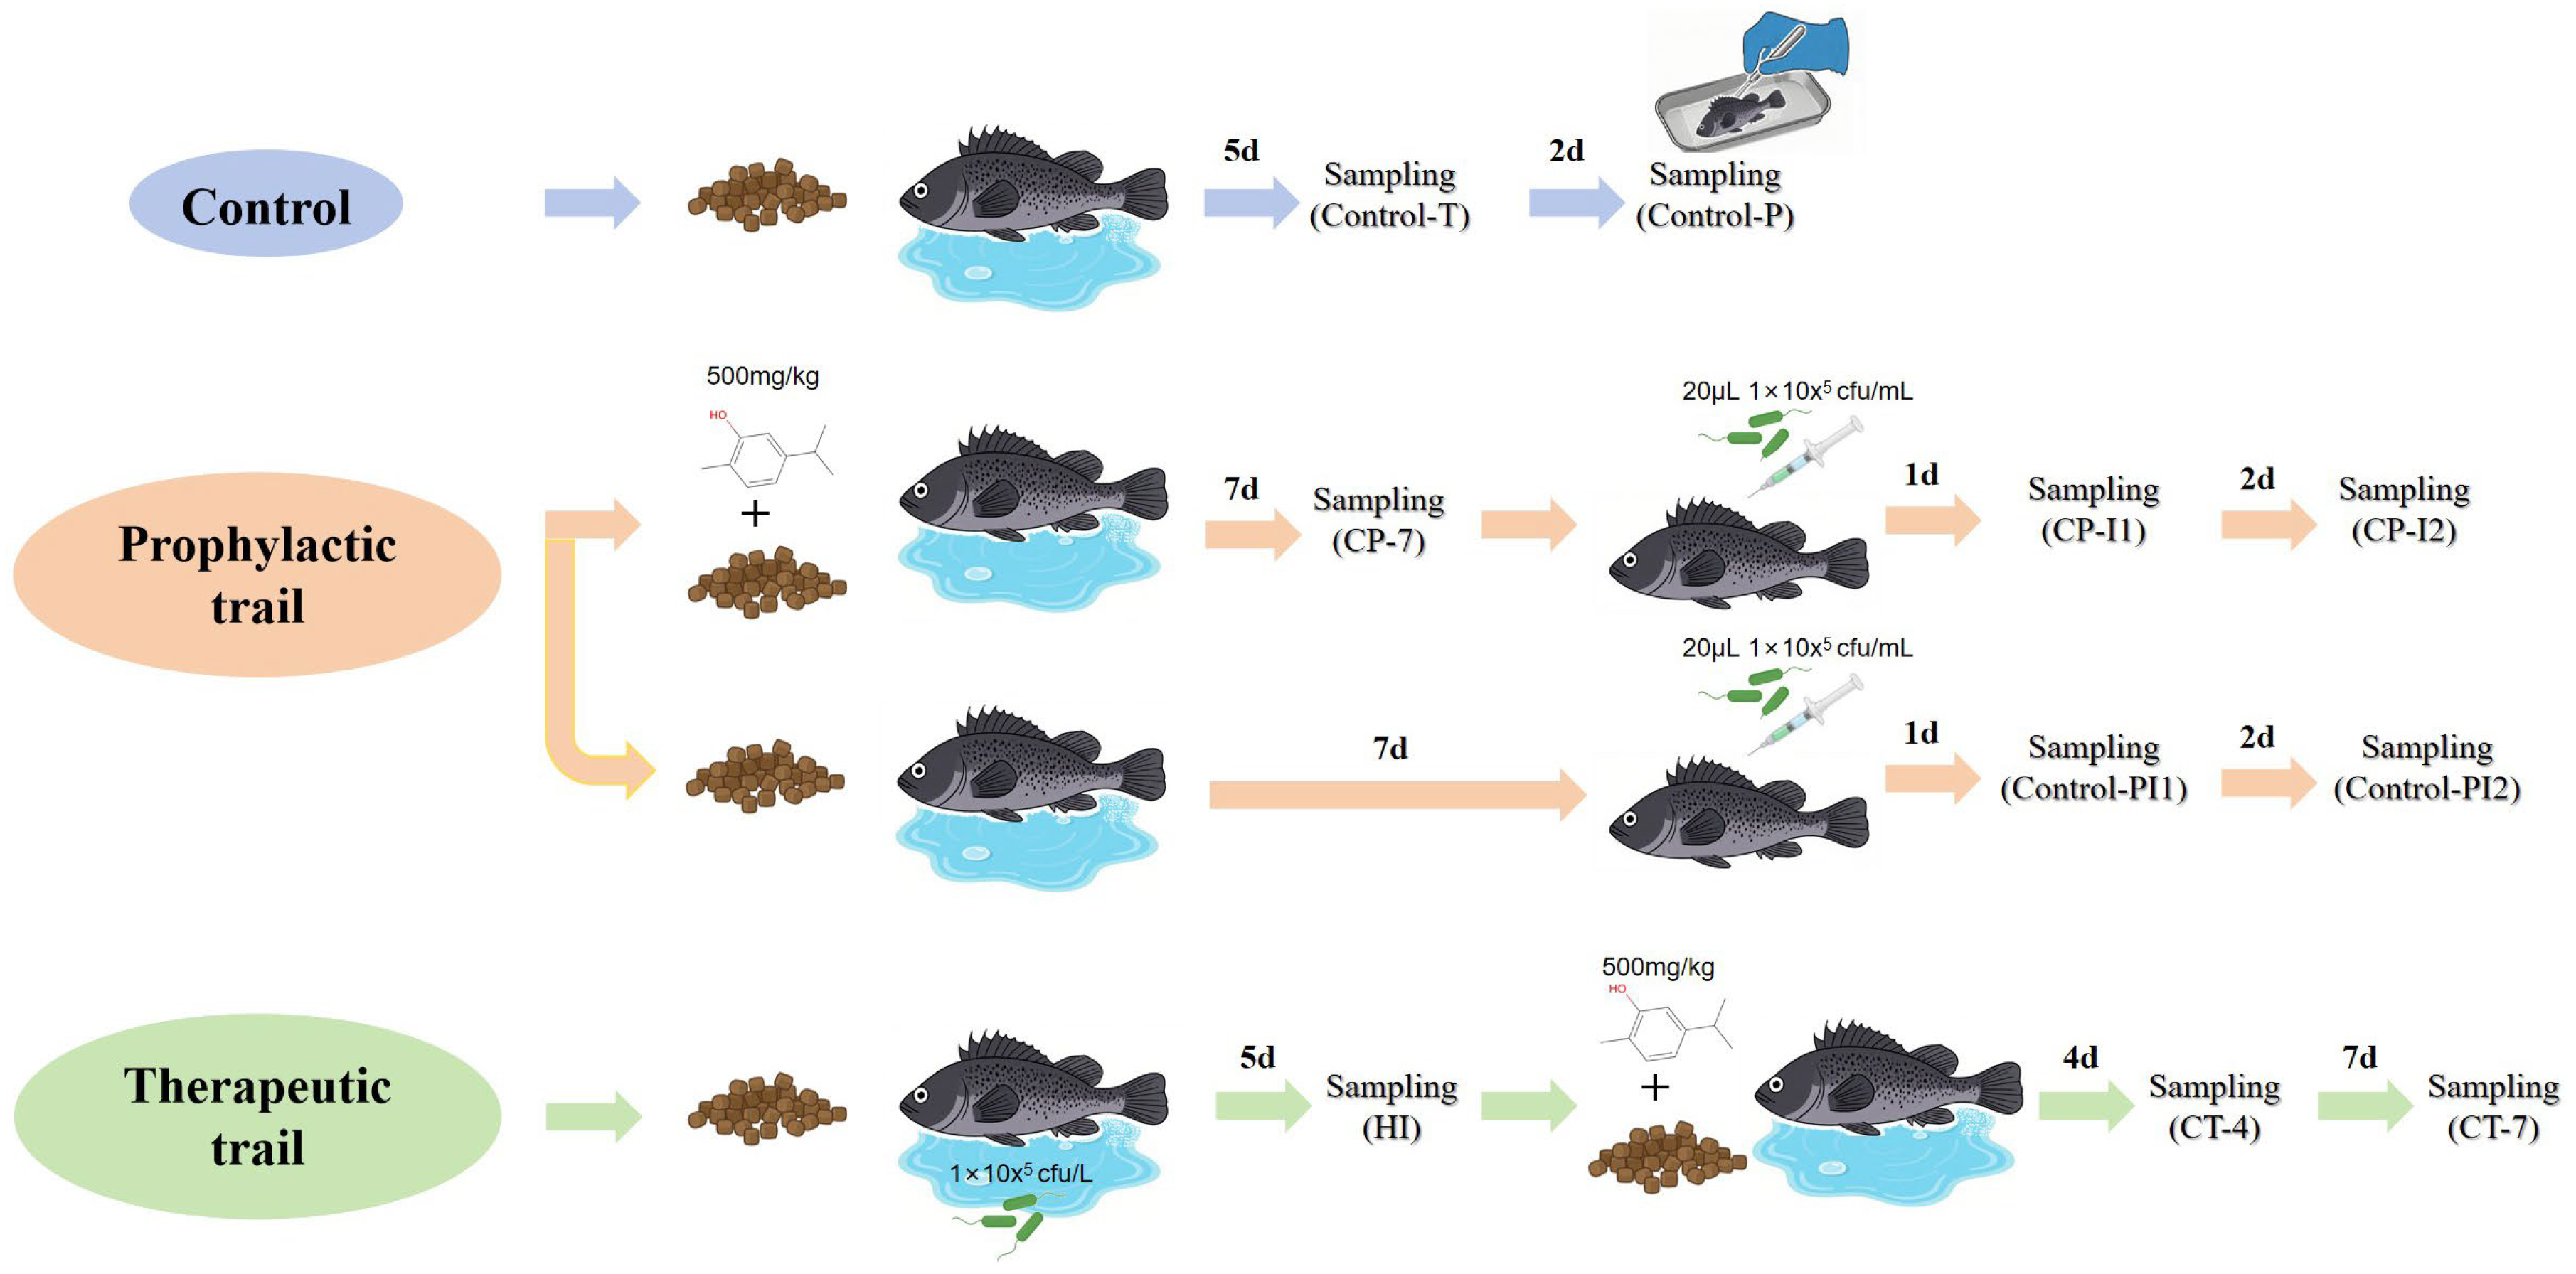
The experiments were conducted at an aquaculture facility in Rizhao, Shandong Province. S. schlegelii fingerlings (body weight of 70 ± 5 g) were acclimated for one week with commercial floating pellets and subjected to a 24 h fasting period before the commencement of the experiment. Throughout the experiment, the water temperature was maintained at 24 ± 2 °C, and one-third of the water in each culture system was replaced daily. To systematically evaluate the immunomodulatory effects of carvacrol and its antagonistic potential against bacterial infection in S. schlegelii, a two-phase experimental framework was designed: prophylactic trail and therapeutic trail (the schematic workflow is detailed in Figure 1). In prophylactic trial, 240 fish were randomly allocated into four net cages (1 m × 1 m × 1 m), with a stocking density of 60 individuals per cage. Two cages were fed a basal control diet, while the other two cages were administered a diet supplemented with 500 mg/kg carvacrol (Aladdin Biochemical Technology Co., Ltd., Shanghai, China) premix. After 7 days of feeding, one net cage from each dietary group was randomly selected for sampling (designated as Control-P and CP-7, respectively), while the remaining two cages were intramuscularly injected with 20 μL of V. harveyi suspension (1 × 10⁵ CFU/mL, prepared in sterile PBS). Subsequently, tissue samples were collected at 1 and 2 days post-injection (designated as Control-PI1/2 and CP-I1/2, respectively). In therapy trial, 120 fish were distributed into four plastic tanks (1 m × 0.8 m × 0.4 m), with 30 individuals per tank. An immersion challenge was performed by inoculating the rearing water with V. harveyi at a final concentration of 1 × 10⁵ CFU/L. Five days post-challenge, fish from two random tanks were sampled (designated as HI), while the remaining two tanks were treated with a diet mixed with 500 mg/kg carvacrol. Then, tissue samples were collected on day 4 (CT-4) and day 7 (CT-7) of the therapeutic treatment period, respectively. Throughout the V. harveyi challenge period in the experiment, the apparent symptoms of the experimental fish were continuously recorded. Concurrently, the daily mortality was documented, and the survival rate was calculated using the following formula:
S u r v i v a l   R a t e   =   T o t a l   f i s h     d e a d   f i s h T o t a l   f i s h   ×   100 %
Following the completion of survival monitoring, the remaining fish were euthanized and dissected for the subsequent physiological and molecular assays. In all groups except Control-PI1 and CP-I1, the foregut was harvested for microbial community profiling, the hindgut was collected for untargeted metabolomic analysis, the midgut was fixed for histopathological examination. In all groups the midgut was preserved for transcriptomic quantification of immune-related genes, the liver was excised for the assessment of antioxidant and metabolic enzyme activities. Furthermore, liver, spleen, and head kidney tissues were separately collected from fish in the CP-7 and Control-P, and fixed in Universal tissue fixative (10% neutral buffered formalin, Servicebio, Wuhan, China) for subsequent immunohistochemical assays. Peripheral blood was collected and processed for leukocyte separation, followed by flow cytometric analysis to evaluate the effects of carvacrol on specific immune responses in S. schlegelii.

2.3. Histopathological Examination

Intestinal samples used for pathological sectioning were fixed in Davidson’s fixative (220 mL HCHO, 330 mL C2H5OH, 115 mL CH3COOH, 335 mL H2O) for 16 h and then transferred to 75% ethanol (Sinopharm Chemical Reagent Co., Ltd., China). Subsequently, tissues were serially dehydrated in the graded ethanol, cleared in xylene (Sinopharm Chemical Reagent Co., Ltd., China), and infiltrated with liquid paraffin using an ASP300S Tissue Processor (LEICA, Wetzlar, Germany). The processed tissues were embedded in paraffin blocks using an EG1150H embedding center (Leica, Wetzlar, Germany). After trimming, the paraffin blocks were sectioned to a thickness of 5 μm with an RM2235 Rotary Microtome (LEICA, Wetzlar, Germany), and a minimum of three non-consecutive sections was prepared per block to ensure representativeness. Tissue sections were transferred onto glass slides and gently stretched by gradually adding 30% ethanol along the slide edges. Slides were placed on an HI1220 slide dryer (Leica, Wetzlar, Germany) and maintained at 45 °C to achieve complete flattening of sections, followed by drying at 60 °C for 10 h to enhance tissue adhesion. Finally, mounted sections were subjected to hematoxylin and eosin (H & E) staining using an AUTO SSTAINER XL automated stainer (Leica, Wetzlar, Germany).

2.4. Carvacrol Treatment and Intestinal Pathogen Load in Sebastes schlegelii

Two complementary strategies were employed for microbial diversity profiling in this study: DNA-based sequencing and RNA reverse transcription-based sequencing. DNA-based sequencing enables the comprehensive capture of total microbial communities, encompassing both viable and dead cells within the sample. In contrast, RNA-based sequencing specifically targets metabolically active and transcriptionally competent microorganisms. High-throughput sequencing for both approaches was performed by Shanghai Meiji Biomedical Technology Co., Ltd., Shanghai, China. A comparative analysis between the two methodologies was systematically conducted to assess intestinal microbial diversity and functional activity.

2.5. Effects of Carvacrol on Non-Specific Immunity of Sebastes schlegelii Under Vibrio harveyi Stress

To investigate the effects of carvacrol on non-specific immune responses under pathogenic bacterial challenge, the transcript levels of intestinal inflammation-related genes and corresponding enzyme activities were quantified.

2.6. Quantitative Real-Time PCR Analysis

Midgut tissues were retrieved from −80 °C storage, immediately flash-frozen in liquid nitrogen, and ground to a fine powder under liquid nitrogen using a pre-chilled mortar and pestle. Total RNA was extracted using the FastPure Cell/Tissue Total RNA Isolation Kit V2 (Vazyme Biotech Co., Ltd., Nanjing, China). RNA concentration and purity were determined using a NanoDrop spectrophotometer (Thermo Fisher Scientific, Waltham, MA, USA), and cDNA was immediately synthesized using the HiScript III RT SuperMix for qPCR (+gDNA wiper) kit (Vazyme, Nanjing, China). Subsequently, qPCR was performed using the Taq Pro Universal SYBR qPCR Master Mix (Vazyme, Nanjing, China). Three target genes associated with inflammatory responses were selected for expression analysis, with RPL-17 employed as the internal reference gene. The annealing temperature was set at 58–62 °C to meet the instrument program requirements, and the amplicon size was set at 80–250 bp to ensure amplification efficiency. Gene sequences were obtained from the NCBI database, and primers were designed using Primer Premier 5 software. The specific qPCR primer sequences are listed in Table 1. F stands for the forward primer, and R stands for the reverse primer.

2.7. Determination of Enzyme Activities

Midgut tissues of S. schlegelii were harvested from −80 °C storage and immediately flash-frozen in liquid nitrogen to maintain tissue integrity and stabilize endogenous enzymatic activities. The concentrations of total protein (TP) and malondialdehyde (MDA), as well as the enzymatic activities of alkaline phosphatase (AKP), acid phosphatase (ACP), catalase (CAT), and superoxide dismutase (SOD), were accurately determined using commercial assay kits according to the manufacturer’s protocols (Nanjing Jiancheng Bioengineering Institute, Nanjing, China).

2.8. Regulatory Effect of Carvacrol Prophylactic Treatment on Specific Immunity in Sebastes schlegelii

2.8.1. Immunohistochemical Analysis

To evaluate the modulatory effects of a 7-day prophylactic administration of carvacrol on the specific immune response of S. schlegelii, immunohistochemistry and flow cytometry were performed to characterize the adaptive immune response. Liver, spleen, and head-kidney specimens were fixed for 24 h, processed into paraffin sections, and subjected to dewaxing. Endogenous peroxidase activity was quenched using 3% hydrogen peroxide (Sinopharm Chemical Reagent Co., Ltd., Shanghai, China) in the dark for 25 min. Tissue Sections were blocked with 3% bovine serum albumin (BSA, Thermo Scientific, Waltham, MA, USA) for 30 min, followed by sequential incubation with primary and secondary antibodies. The rigorously validated antibodies (1:10,000 dilution) targeting CD4-1, CD79a, and CD79b proteins were used as the primary antibody, respectively. Horseradish peroxidase (HRP)-conjugated goat anti-rabbit IgG (1:50,000 dilution, Jackson ImmunoResearch Inc., Lancaster, PA, USA, USA) served as the secondary antibody. Immunoreactivity was visualized using 3,3′-diaminobenzidine (DAB, Solarbio, Beijing, China) chromogen, and nuclei were counterstained with hematoxylin (Solarbio, Beijing, China). After dehydration, clearing, and mounting, slides were examined microscopically, and the number and proportion of positively stained immune cells were recorded for comparative analysis.

2.8.2. Flow Cytometric Sorting of Peripheral Blood Lymphocytes

Prior to blood collection, 4 mL of single-cell suspension medium was aspirated into a 5 mL sterile syringe. Six fish were randomly selected from each group and subjected to caudal vein blood collection, with samples immediately transferred into sterile 15 mL centrifuge tubes. Leukocyte isolation was performed within 2 h using a commercial fish peripheral blood leukocyte isolation kit (Tianjin Haoyang Biological Products Technology Co., Ltd., Tianjin, China) according to the manufacturer’s instructions. The obtained leukocytes were incubated with the aforementioned prepared primary antibodies (1:10,000 dilution) at room temperature with shaking at 100 rpm for 1 h. After centrifugation and washing with ice-cold 1% BSA-PBS, cells were incubated with a 488-labeled secondary antibody (1:1000 dilution, Hangzhou Start Biotechnology Co., Ltd., Hangzhou, China) in the dark for 1 h. Samples were then washed and filtered through a 40-μm cell strainer prior to flow cytometric analysis. Antibody-labeled cells were resuspended in ice-cold PBS at a density of 1 × 10⁶–1 × 10⁷ cells/mL and analyzed using a Beckman CytoFLEX flow cytometer (Beckman Coulter, Inc., Brea, CA, USA) with the fluorescein isothiocyanate (FITC) fluorescence channel. Data acquisition was performed until 10,000 events were recorded per sample, and all data were stored for subsequent statistical analysis.

2.9. Statistical Analysis

Statistical analyses were performed using SPSS (IBM SPSS Statistics 27.0.1) and the Meiji Cloud Platform (Shanghai Meiji Biomedical Technology Co., Ltd.). One-way Analysis of Variance (ANOVA) or Kruskal–Wallis test were applied to determine statistically significant differences among treatment groups.
The use of experimental animals and the study protocol were reviewed and approved by the Ethics Committee of Yellow Sea fishery research institute, Chinese Academy of Fishery Sciences (Approval No.: YSFRI-2024059, Approval Date: 27 April 2024).

3. Result

3.1. Effects of Carvacrol on Survival and Intestinal Histopathology of Fish Infected with Vibrio harveyi

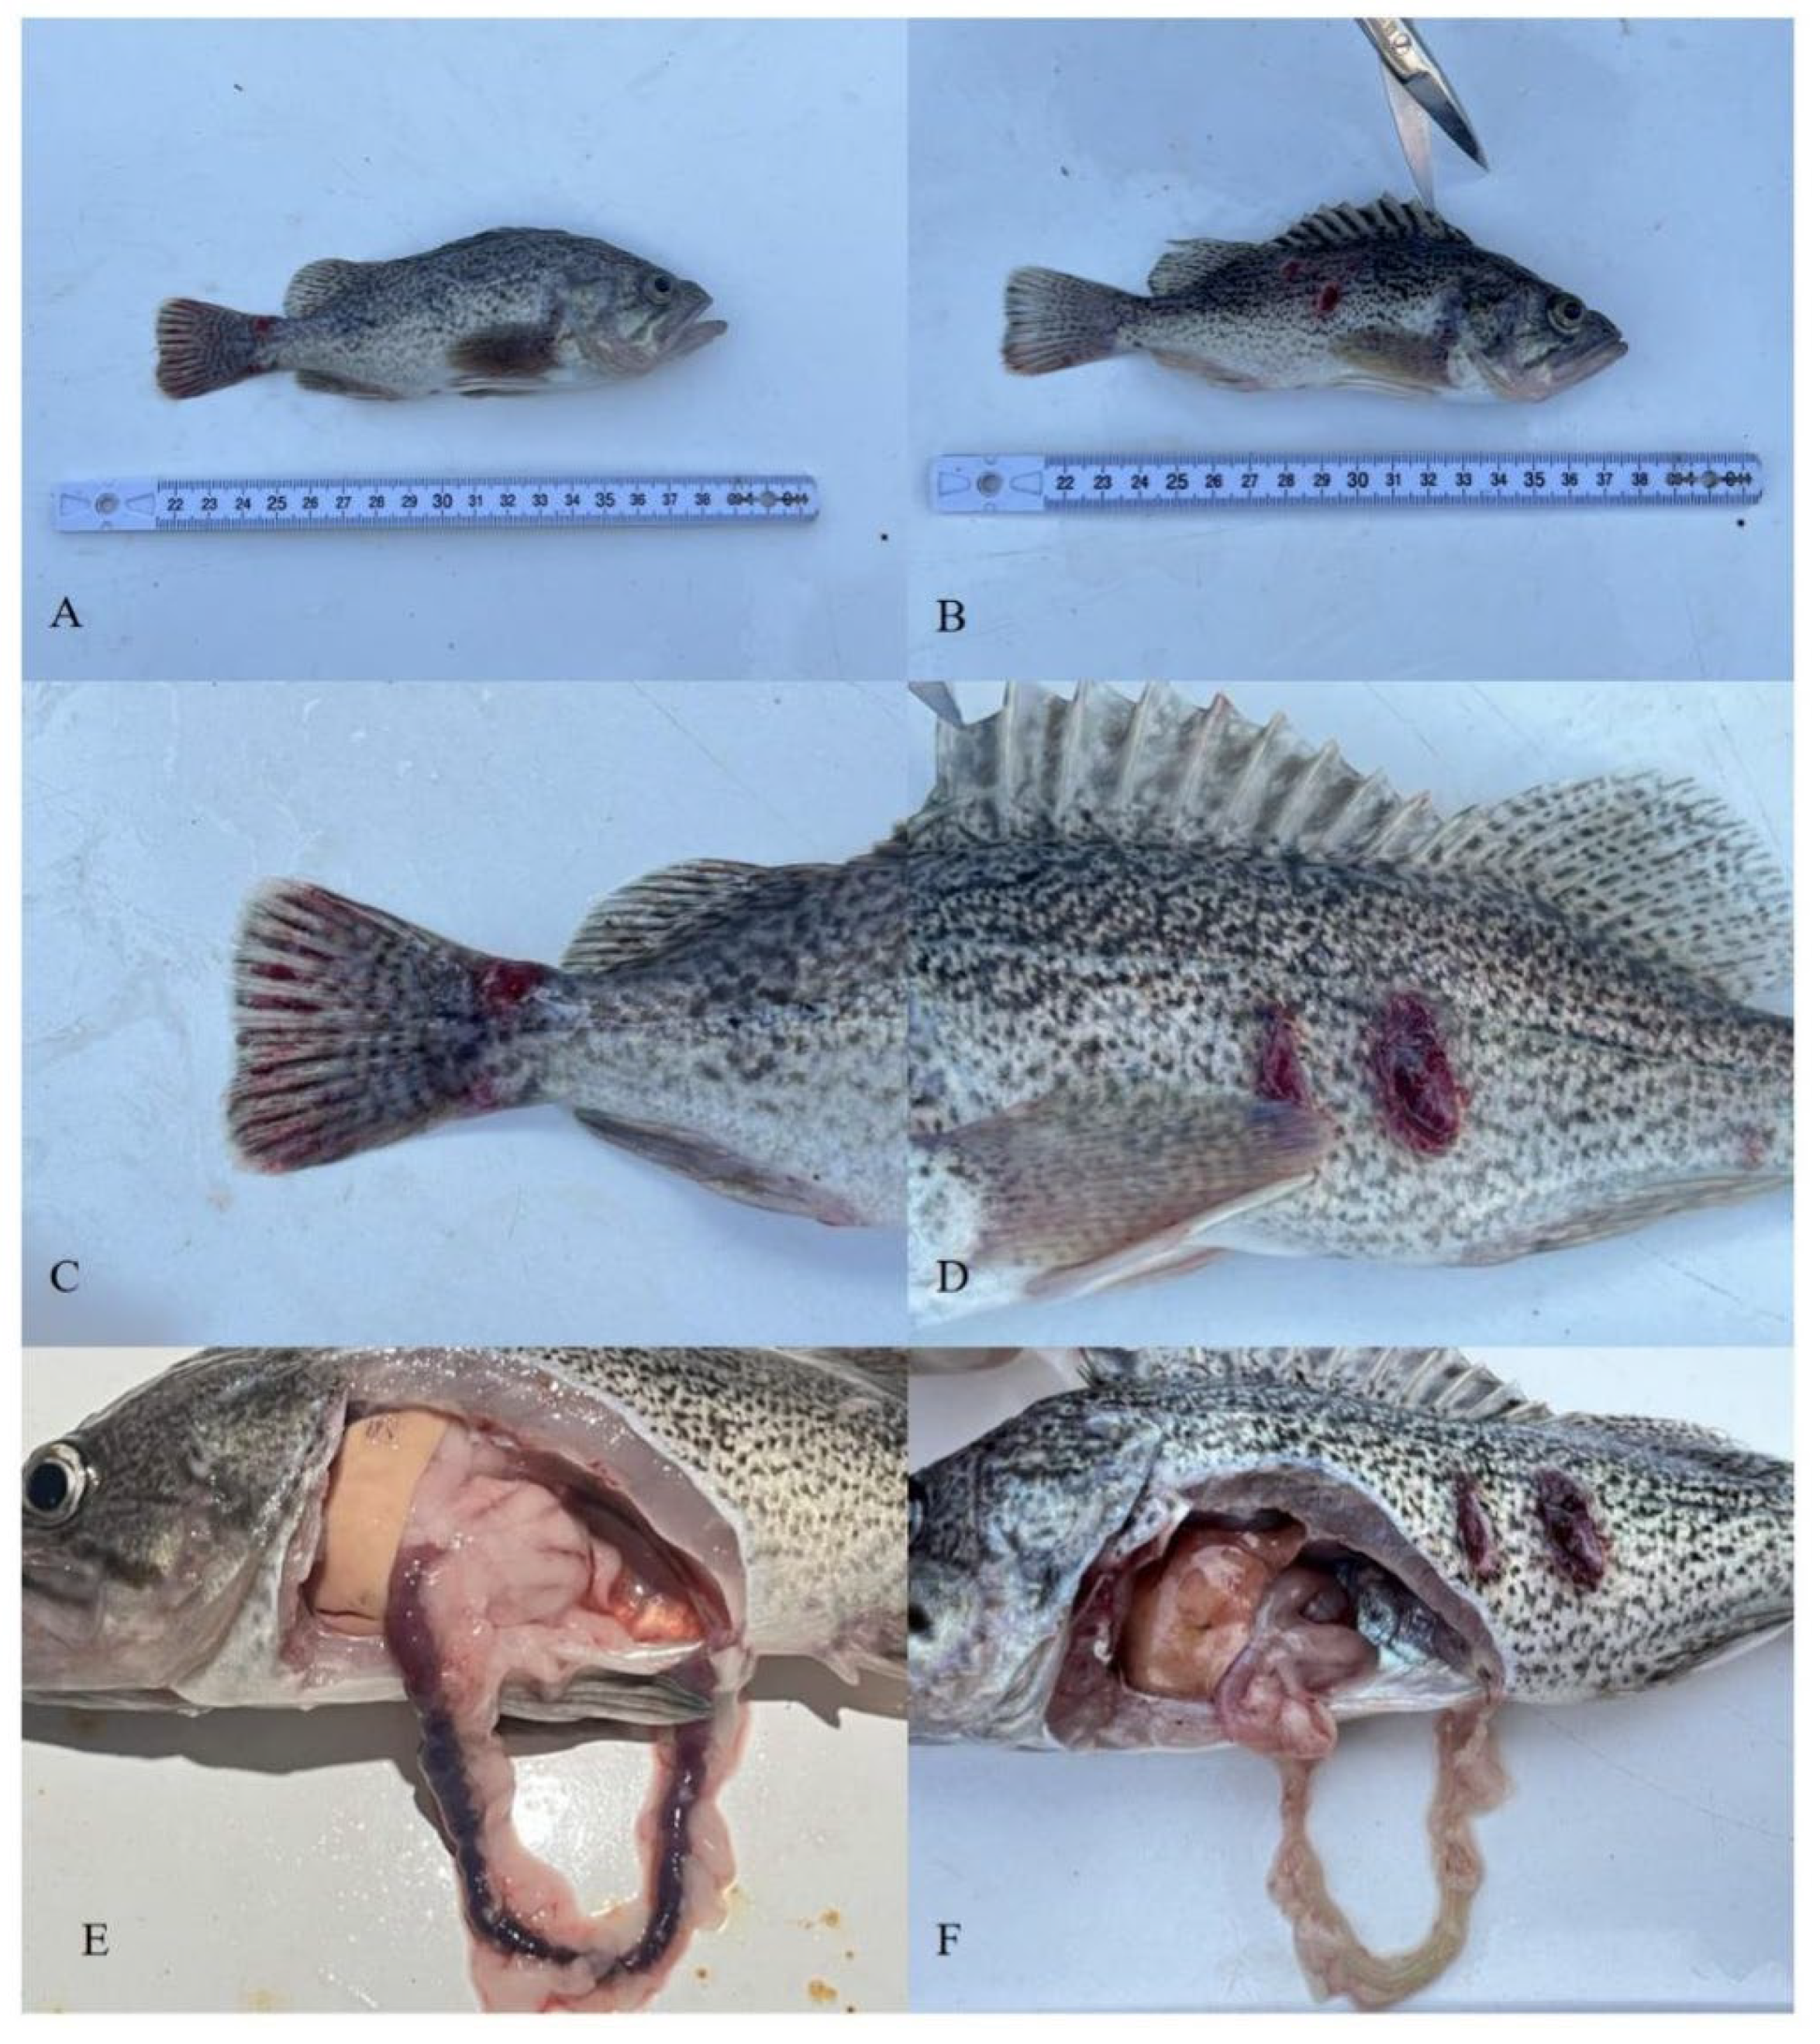
After a 7-day acclimation period with a control diet, the experimental fish subjected to intraperitoneal challenge with V. harveyi for two days (Control-PI2) exhibited severe intestinal hemorrhage. The experimental fish exposed to V. harveyi via immersion challenge for five days (HI) developed characteristic pathological symptoms, including extensive ulceration of the body surface, intestinal hemorrhage, ascites, and significant hepatic atrophy (Figure 2).
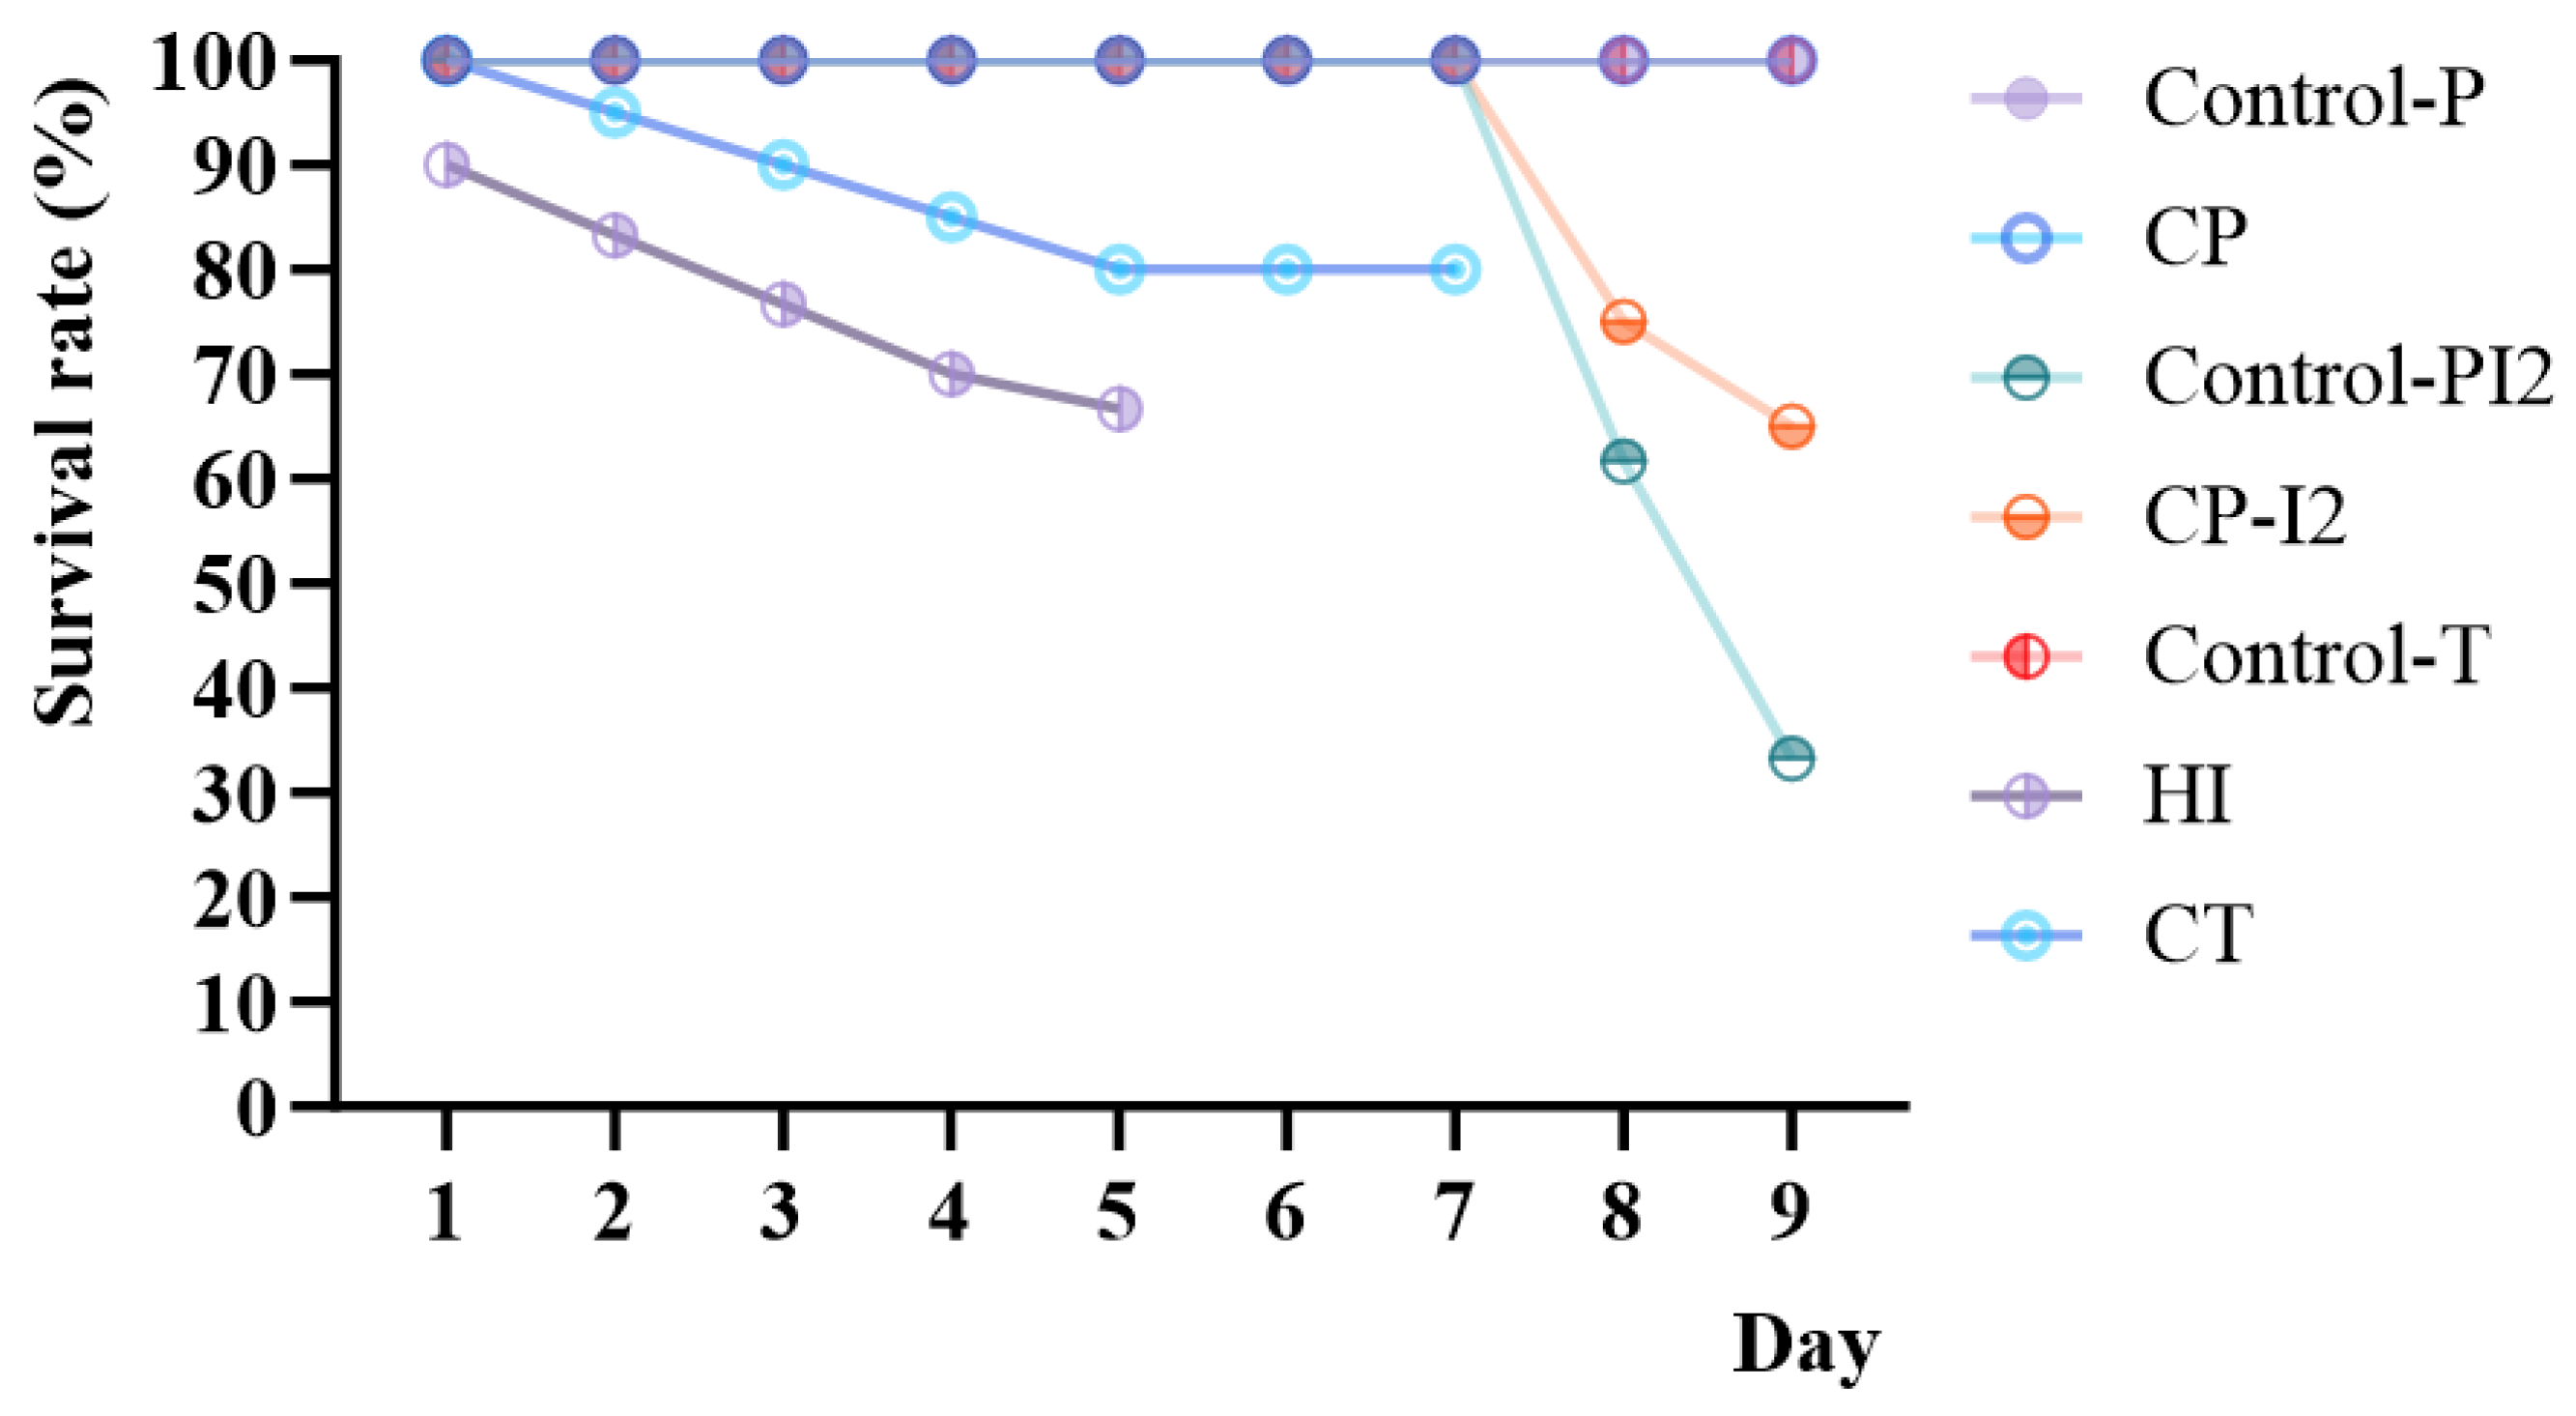
Cumulative survival rates of all experimental groups are presented in Figure 3. Throughout the entire experimental period, no mortality was observed in the Control-P group, Control-T group and the CP-7 group, resulting in a 100% survival rate for all three groups. In the prophylactic trial, fish in the Control-PI2 group exhibited a cumulative survival rate of 33.33%. In contrast, fish in the CP-I2 group showed a markedly higher survival rate of 65%. In the therapeutic trial, fish in the HI had a cumulative survival rate of 66.67%. The carvacrol-treated group (CT) achieved a final cumulative survival rate of 80% following the same immersion challenge, indicating a protective effect of carvacrol against V. harveyi infection.
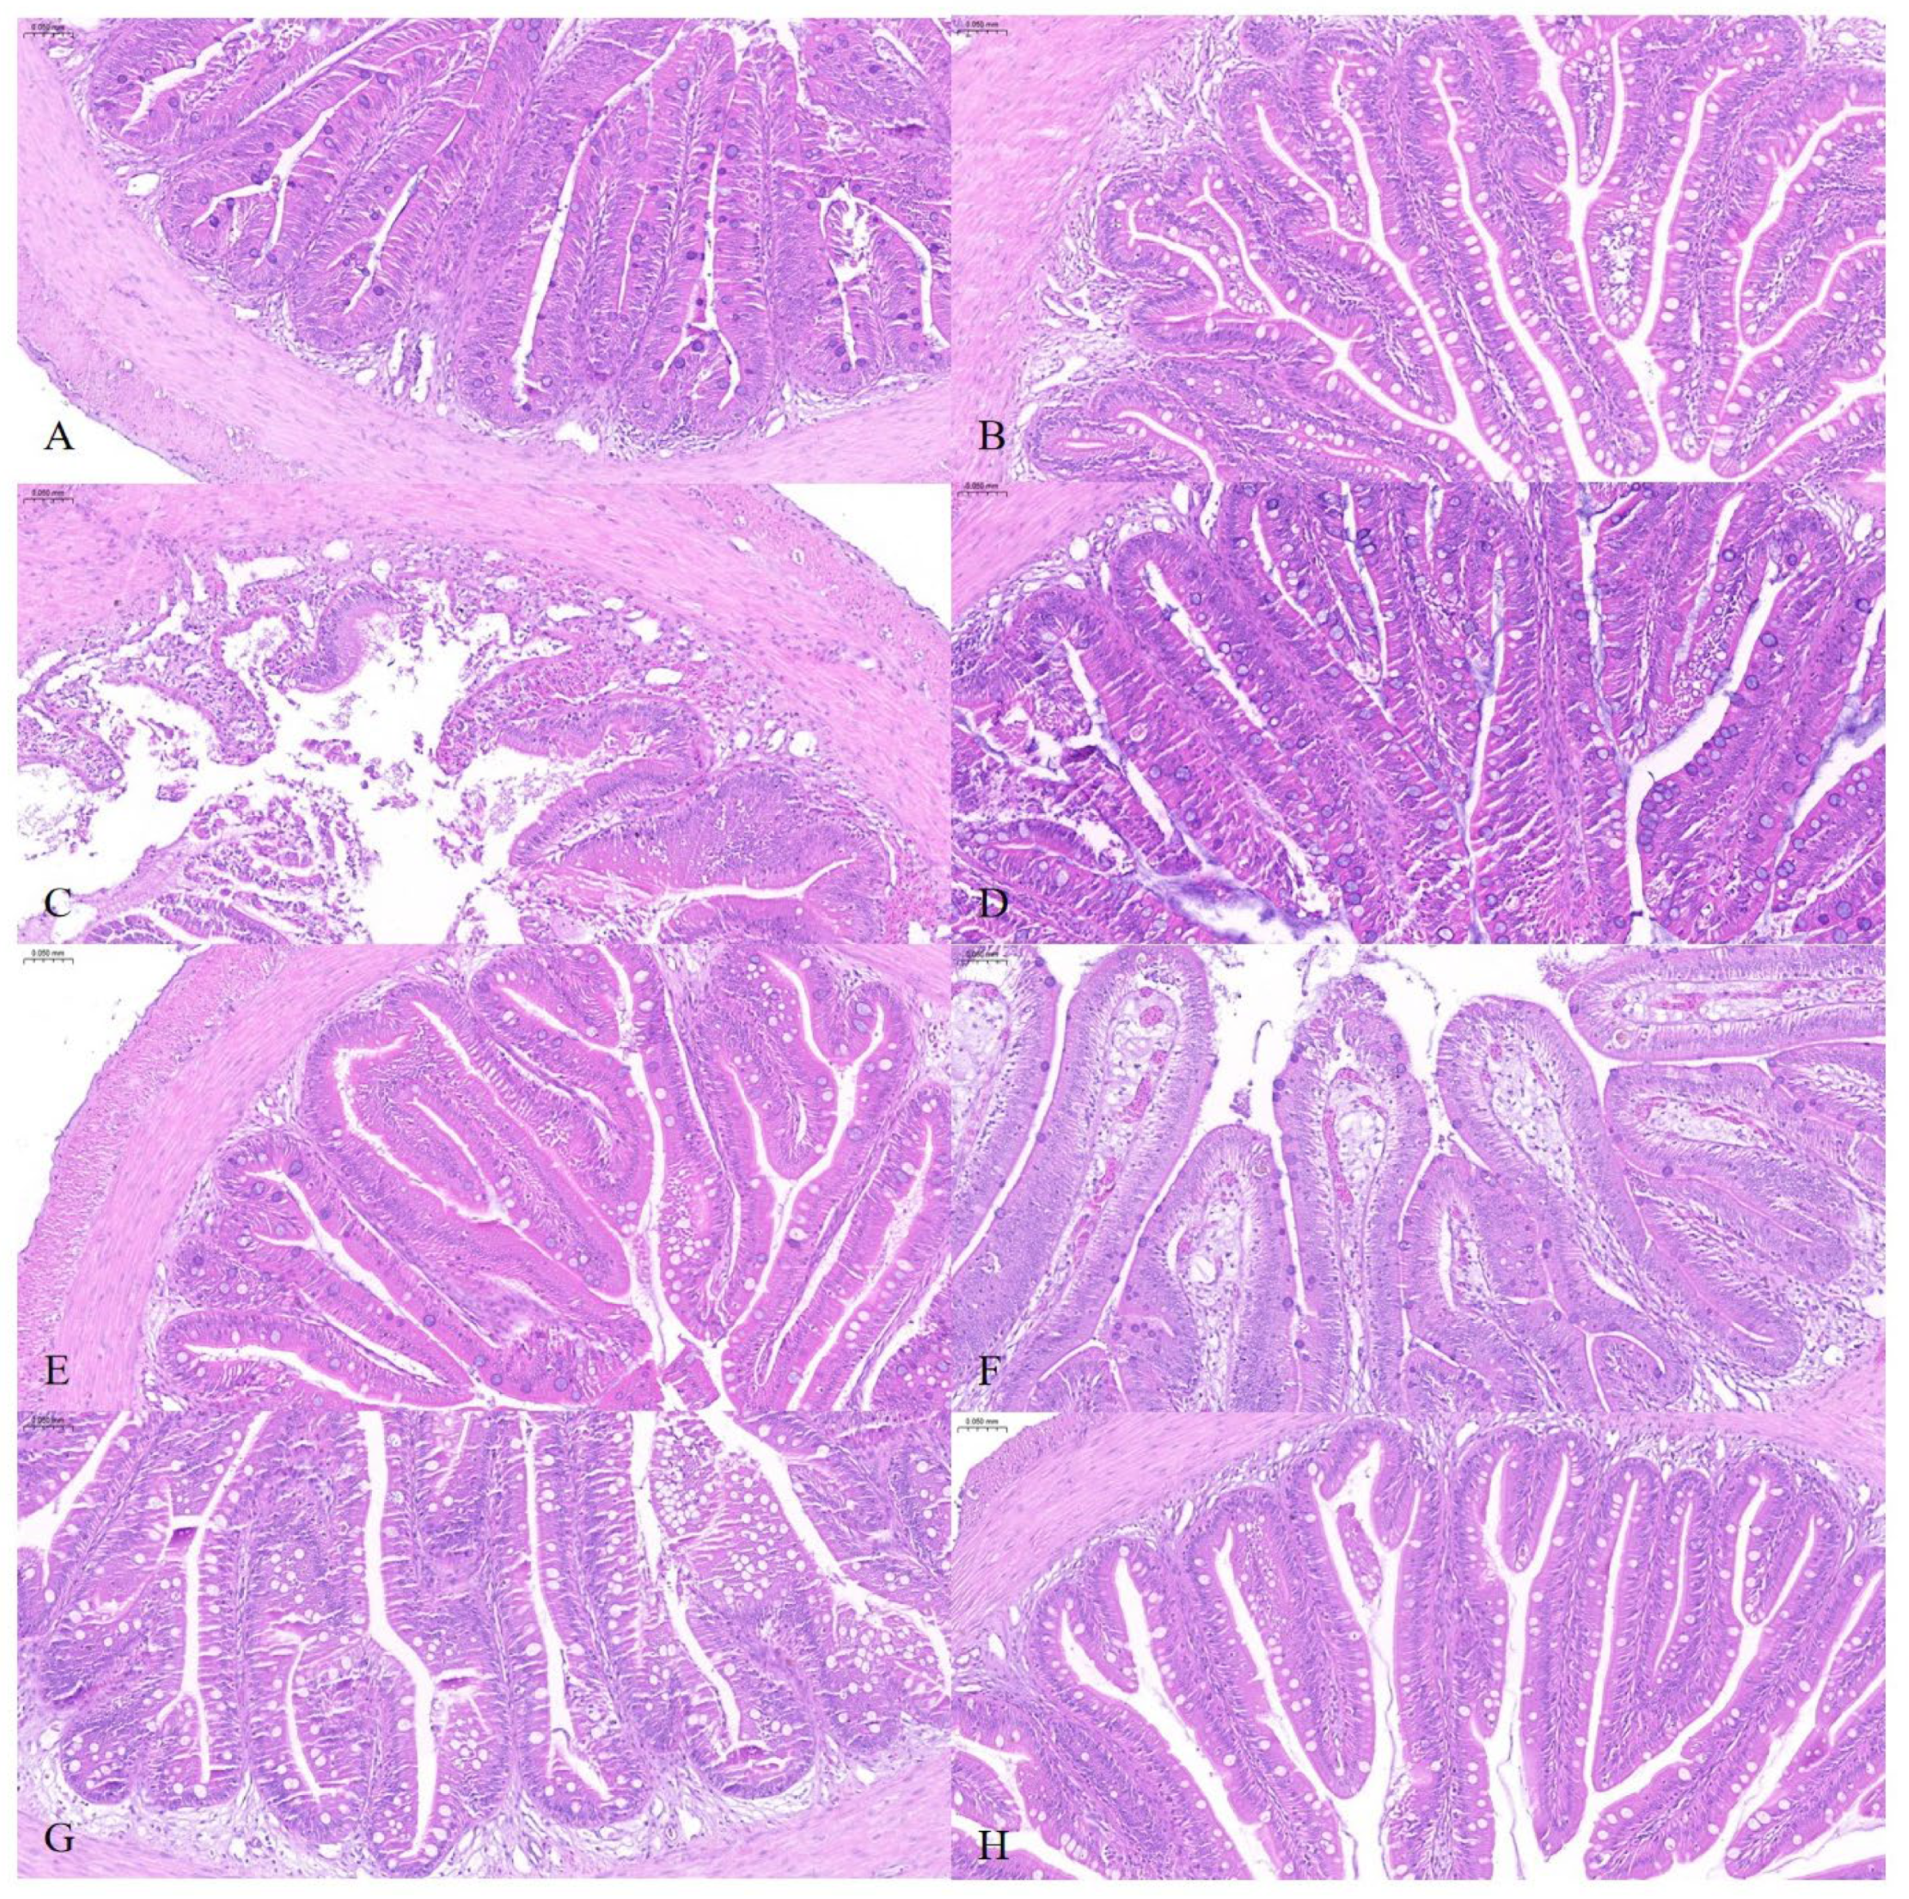
Histopathological observations of intestinal tissues are shown in Figure 4. In the two control groups (Control-P and Control-T), the intestinal mucosa maintained a normal histological architecture. Intestinal villi were dense, structurally intact, and devoid of rupture, fusion, or atrophy. The single-layer columnar epithelial cells were plump with intense cytoplasmic eosinophilia, and their nuclei were regularly aligned at the basal region. Goblet cell density was within normal limits, with no obvious impairment of mucin secretion. The submucosal connective tissue was free of edema and inflammatory cell infiltration. Smooth muscle fibers in the muscular layer were orderly arranged without evidenced hypertrophy or necrosis. The serosal layer remained structurally intact, with no signs of adhesion or exudation. Fish in the Control-PI2 group exhibited extensive fissure-shaped necrotic lesions in the intestinal mucosa. These cavities arose from ischemic or inflammatory necrosis and lysis of mucosal tissues, accompanied by marked infiltration of lymphocytes, macrophages, and other inflammatory cells, together with interstitial edema. In contrast, only mild inflammatory cell infiltration was observed in the intestines in the CP-I2 group. Fish in the HI developed severe intestinal histopathological damage. Intestinal villi showed marked structural disruption and loss of the typical finger-like projections. Columnar epithelial cells were disorganized, with evident vacuolation, focal necrosis, and shedding, leading to interrupted cellular continuity. Goblet cell numbers were decreased and unevenly distributed. The lamina propria exhibited massive inflammatory cell infiltration, accompanied by severe interstitial edema, loosening, and local hyperemia. Fish in the CT-4 group exhibited numerous goblet cells within the intestinal epithelium. Notably, in the CT-7 group, only mild nuclear pyknosis, inflammatory cell infiltration, and edema were detected, with no notable hemorrhage or tissue necrosis.

3.2. Changes in Intestinal Vibrio Load in Sebastes schlegelii Under Pathogen Infection and Carvacrol Treatment

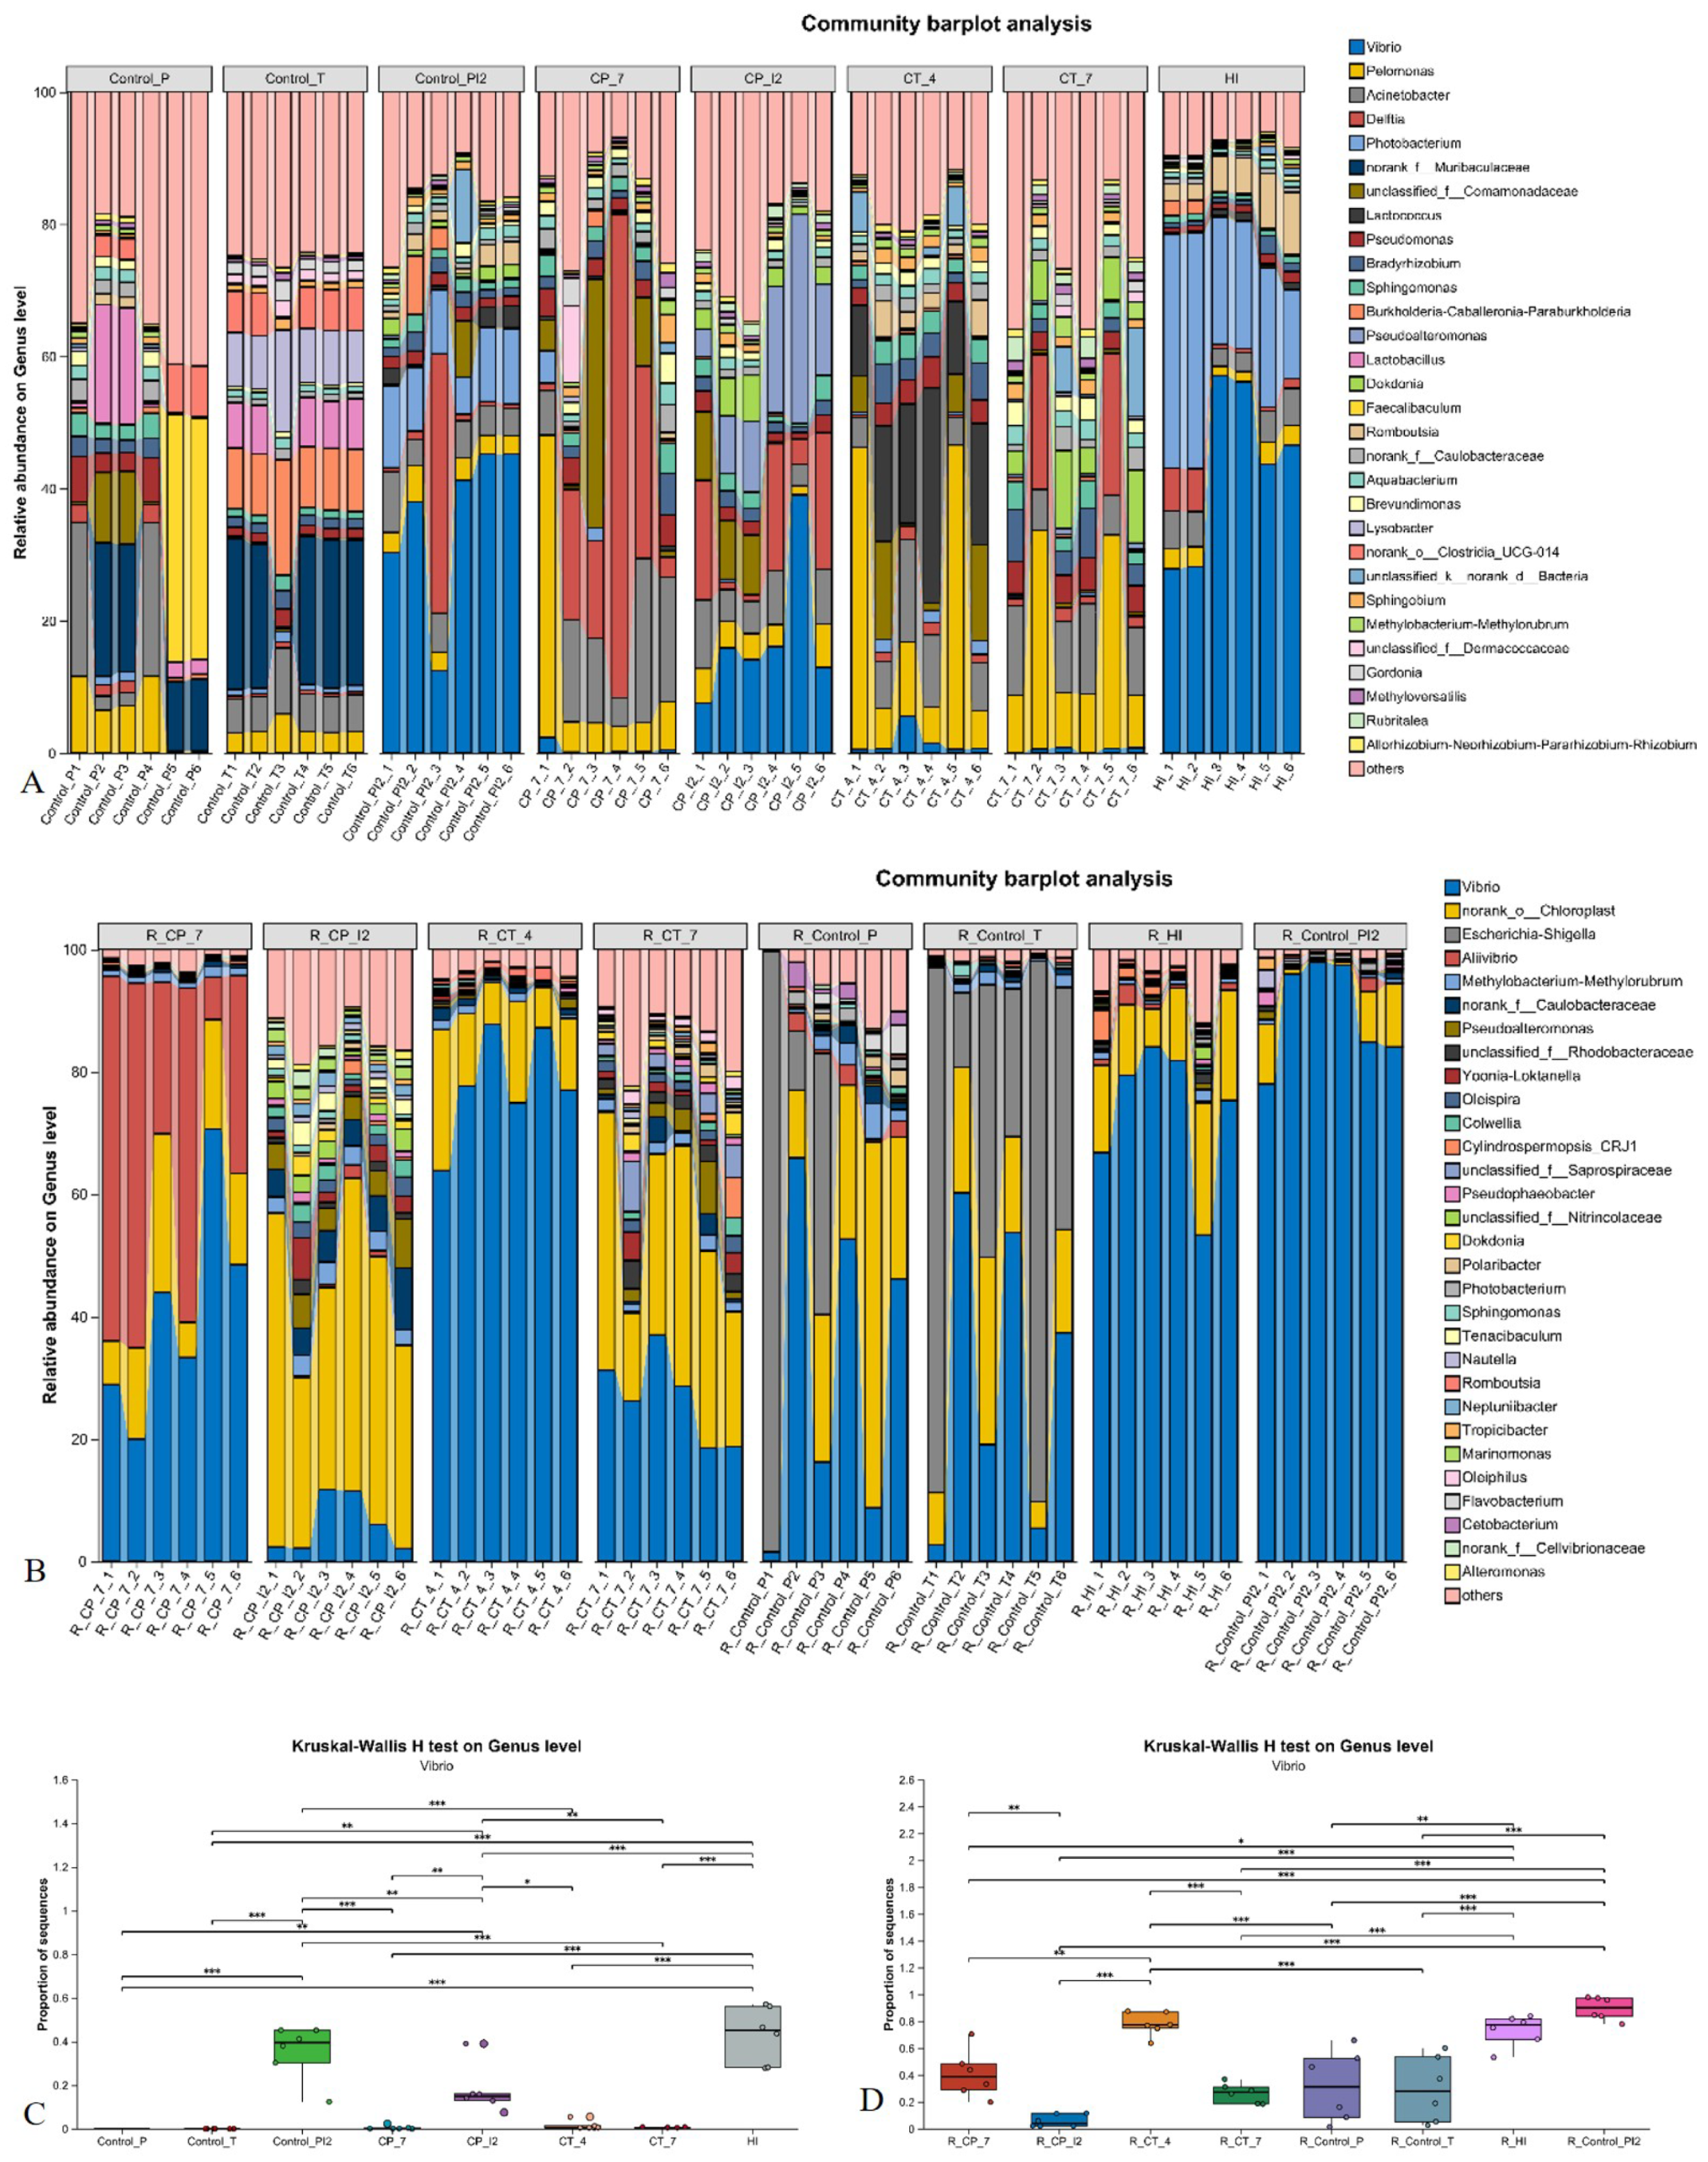
These plots were employed to evaluate the compositional differences between the entire intestinal microbiota and the currently bioactive intestinal microbiota of the experimental fish. The inter-group differences in Vibrio, an important pathogenic genus, are shown in Figure 5C,D.
Vibrio, the predominant pathogen in this study, exhibited intestinal abundance in each experimental fish group, as determined by the two sequencing approaches, as summarized in Table 2. The results indicated that in the prophylactic trial, the intestinal Vibrio loads in fish from the CP-I2 group were significantly reduced by both detection methods when compared with those in the direct challenge group without pretreatment (Control-PI2). In the therapeutic trial, DNA extraction and sequencing method revealed that the intestinal Vibrio loads in fish from the CT-4 group were already significantly decreased compared with that in the immersion challenge group (HI). Meanwhile, the RNA extraction and reverse transcription sequencing method showed that the intestinal Vibrio loads in fish from the CT-7 group.

3.3. Changes in Non-Specific Immunity of Experimental Fish in Each Treatment Group

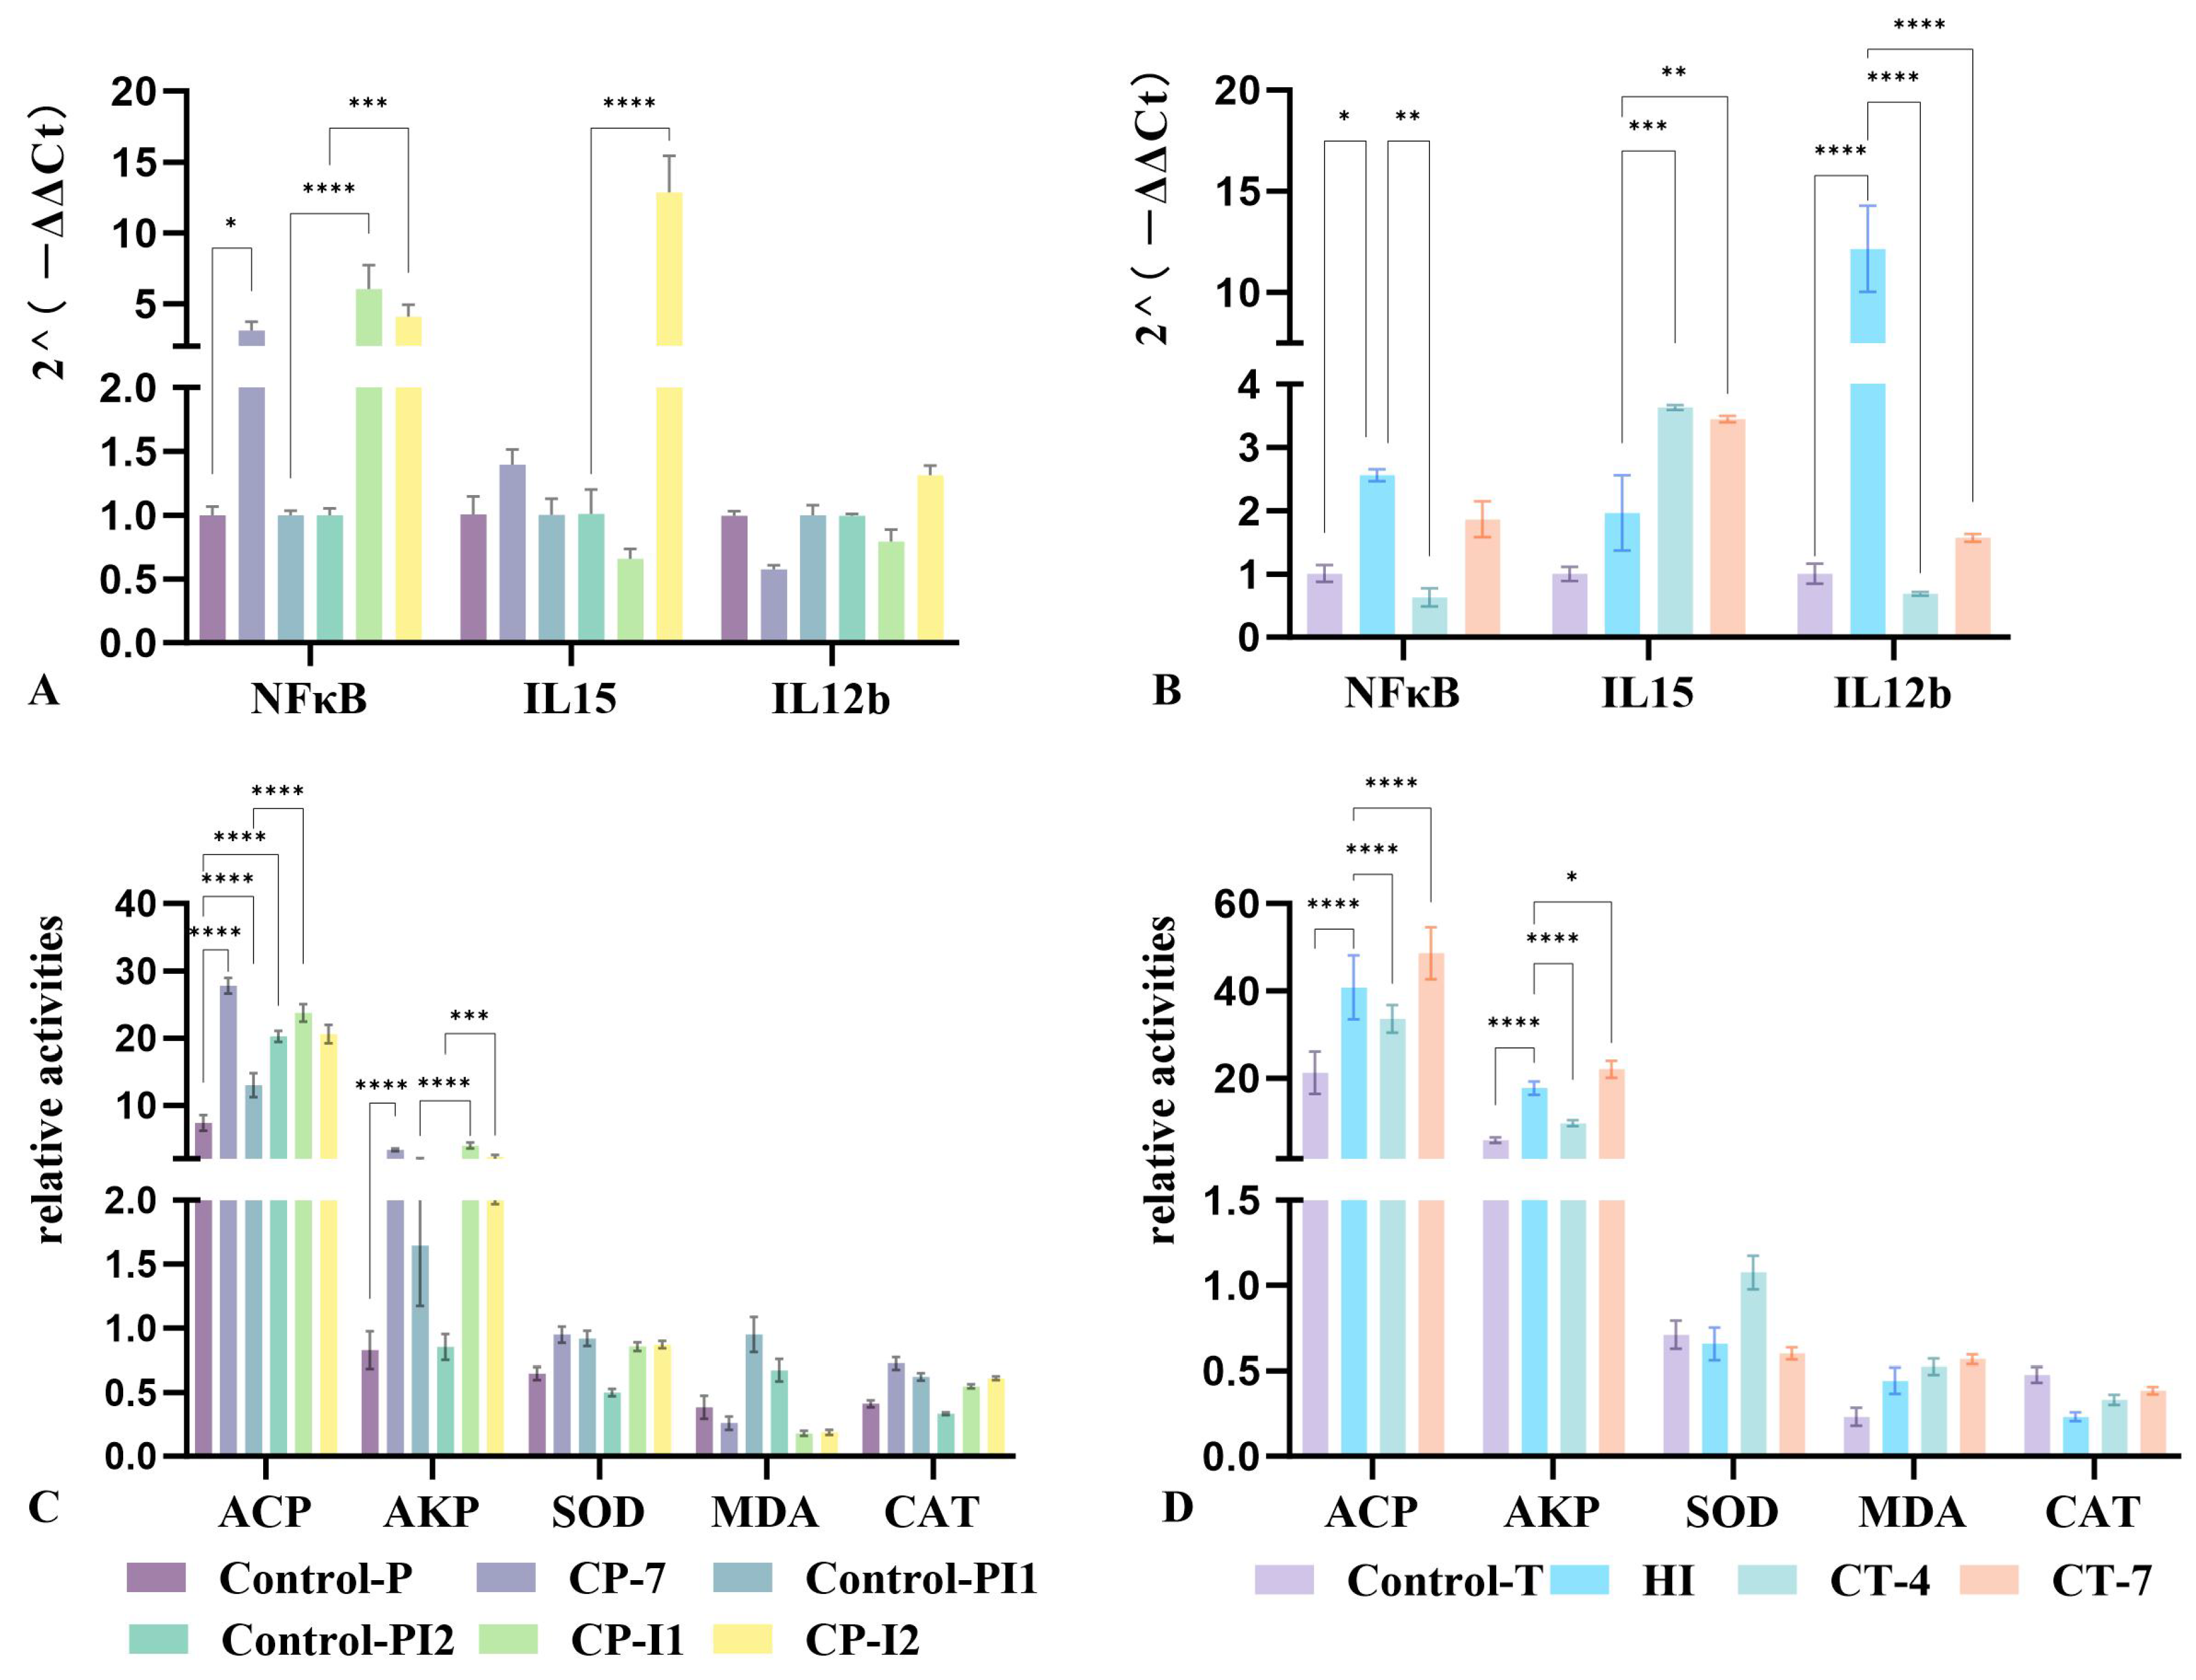
The expression levels of midgut immune genes (NFκB, IL15, and IL12b) and hepatic enzyme activities (ACP, AKP, SOD, CAT, MDA) in experimental fish from different groups are shown in Figure 6. The results indicated that the intestinal expression of NFκB in the CP-7 group was significantly upregulated compared with that in the Control-P. In contrast, there were no significant differences in the expression levels of IL15 and IL12b between the two groups.
For experimental fish in the CP-I1 group and CP-I2 group, the expression of NFκB was significantly upregulated compared to that in the experimental fish from the Control-PI1 group and Control-PI2 group. Additionally, the expression level of IL15 in the CP-I2 group was significantly upregulated compared with that in the Control-PI2 group.
The expression level of NFκB in the HI was significantly upregulated compared to that in the Control-T group. In contrast, the expression level of NFκB after 4-day carvacrol treatment (CT-4) was significantly downregulated compared to the HI group. There was no significant difference in the expression level of IL15 between HI and Control-T. However, the expression levels of IL15 in the CT-4 and CT-7 groups were significantly upregulated when compared to that in the HI group. Regarding IL12b, its expression level in the HI group was significantly upregulated compared to that in the Control-T group, yet the expression levels of IL12b in the CT-4 and CT-7 groups were significantly downregulated compared to that in the HI group.
The activities of AKP, ACP, MDA, CAT and SOD in intestinal tissues sampled under different treatment methods and at different time points are shown in Figure 6C,D. In the prevention phase (Figure 6C), the phosphatase activities (ACP and AKP) of experimental fish in the CP-7 group were significantly upregulated compared to those in the Control-P group. The SOD and CAT activities in the CP-7 group were upregulated relative to the Control-P group, although the difference was not significant. The MDA content in the CP-7 group was downregulated compared to the Control-P group, and this difference was also not statistically significant. The ACP activity in the CP-I1 group was significantly upregulated compared to the Control-PI1 group, while the ACP activity in the CP-I2 group was upregulated compared to theControl-PI2 group, but the difference was not significant. The AKP activities in the CP-I1 and CP-I2 groups were significantly upregulated compared to the Control-PI1 and Control-PI2 groups, respectively. The SOD and CAT activities in the CP-I1 and CP-I2 groups were upregulated compared to their corresponding control groups (Control-PI1 and Control-PI2), but the differences were not significant. The MDA contents in the CP-I1 and CP-I2 groups were downregulated compared to their corresponding control groups, but the differences were not significant. In the treatment section (Figure 6D), the activities of ACP and AKP in experimental fish of the HI were upregulated compared to those in the control group (Control-T). After carvacrol treatment, the activities of ACP and AKP exhibited a trend of significant downregulation first, followed by significant upregulation. There were no significant differences in the activities of SOD, MDA, and CAT among all groups.

3.4. Expression of Specific Immune Cells in Tissues and Peripheral Blood After Prophylactic Administration of Carvacrol

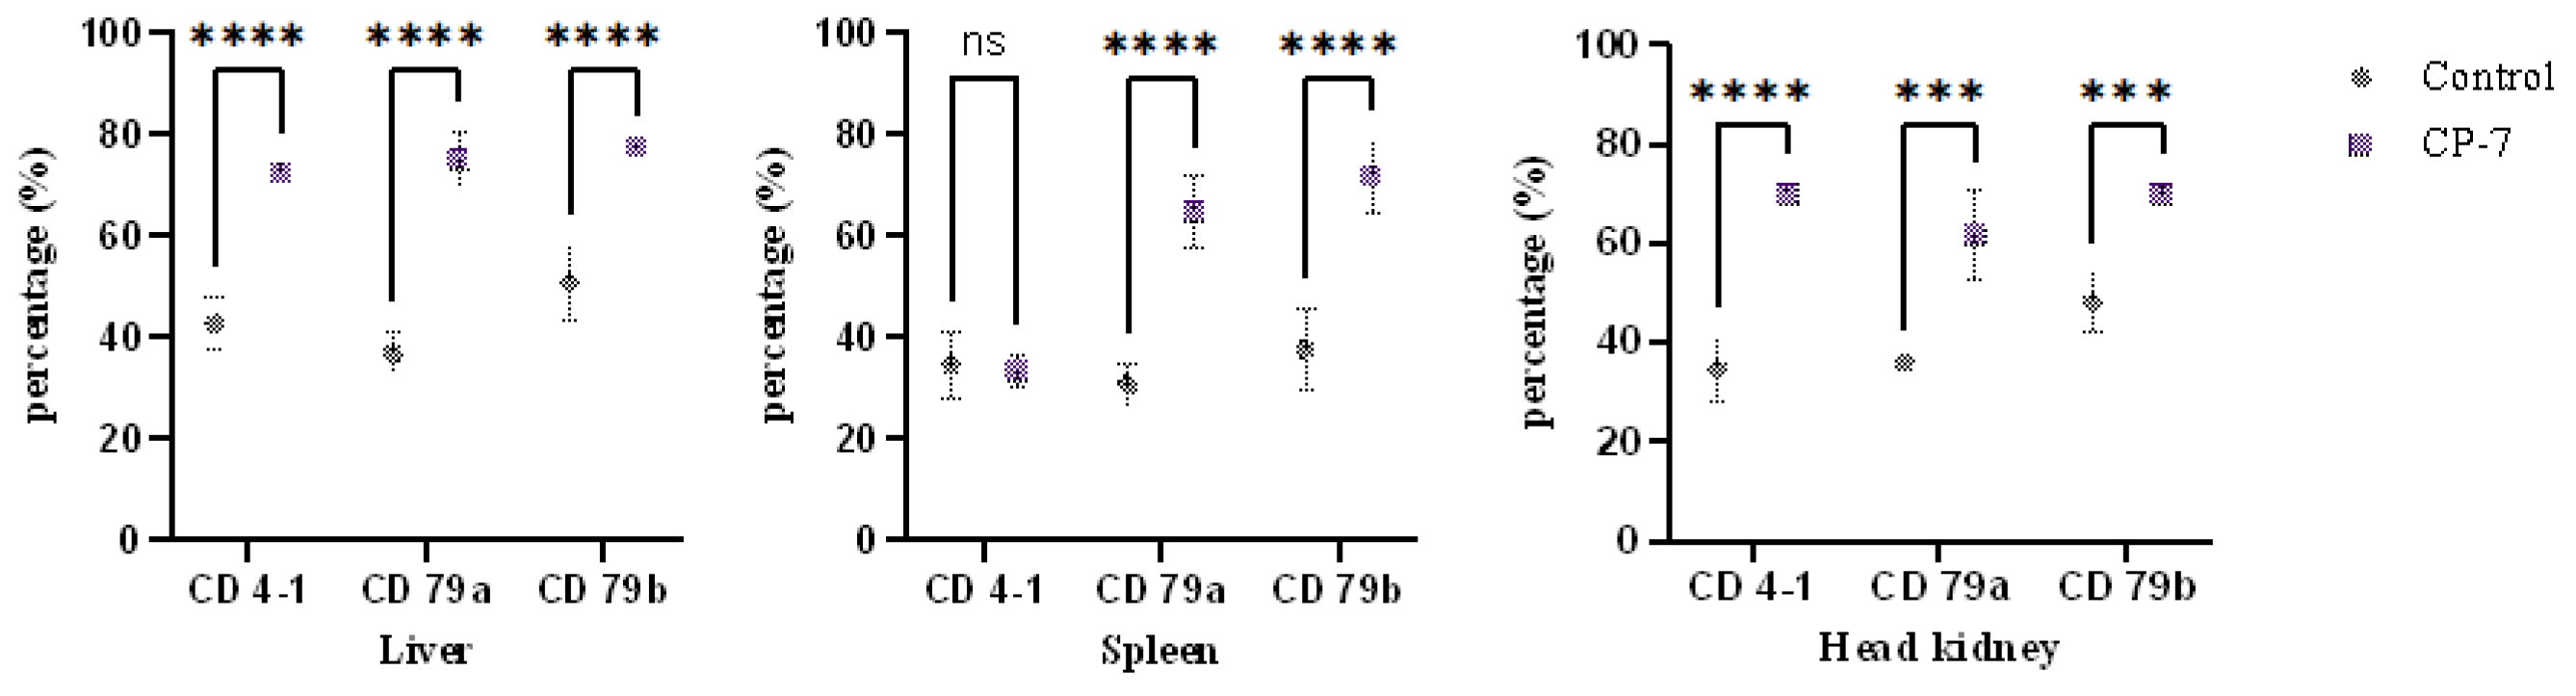
After 7-day prophylactic administration of carvacrol, immunohistochemical assays were performed on the liver, spleen, and head kidney of experimental fish. The percentages of CD4-1+ T cells and CD79a/CD79b+ B cells in the relevant tissues were determined by calculating the ratio of positive cells to total cells in the sections, so as to investigate the effect of carvacrol on specific immunity in experimental fish.
As shown in Figure 7, compared with the Control group, the ratios of CD4-1+ T cells and CD79a/CD79b+ B cells in the liver, CD79a/CD79b+ B cells in the spleen, and CD4-1+ T cells and CD79a/CD79b+ B cells in the head kidney were significantly higher in the fish that were fed carvacrol for prophylaxis.
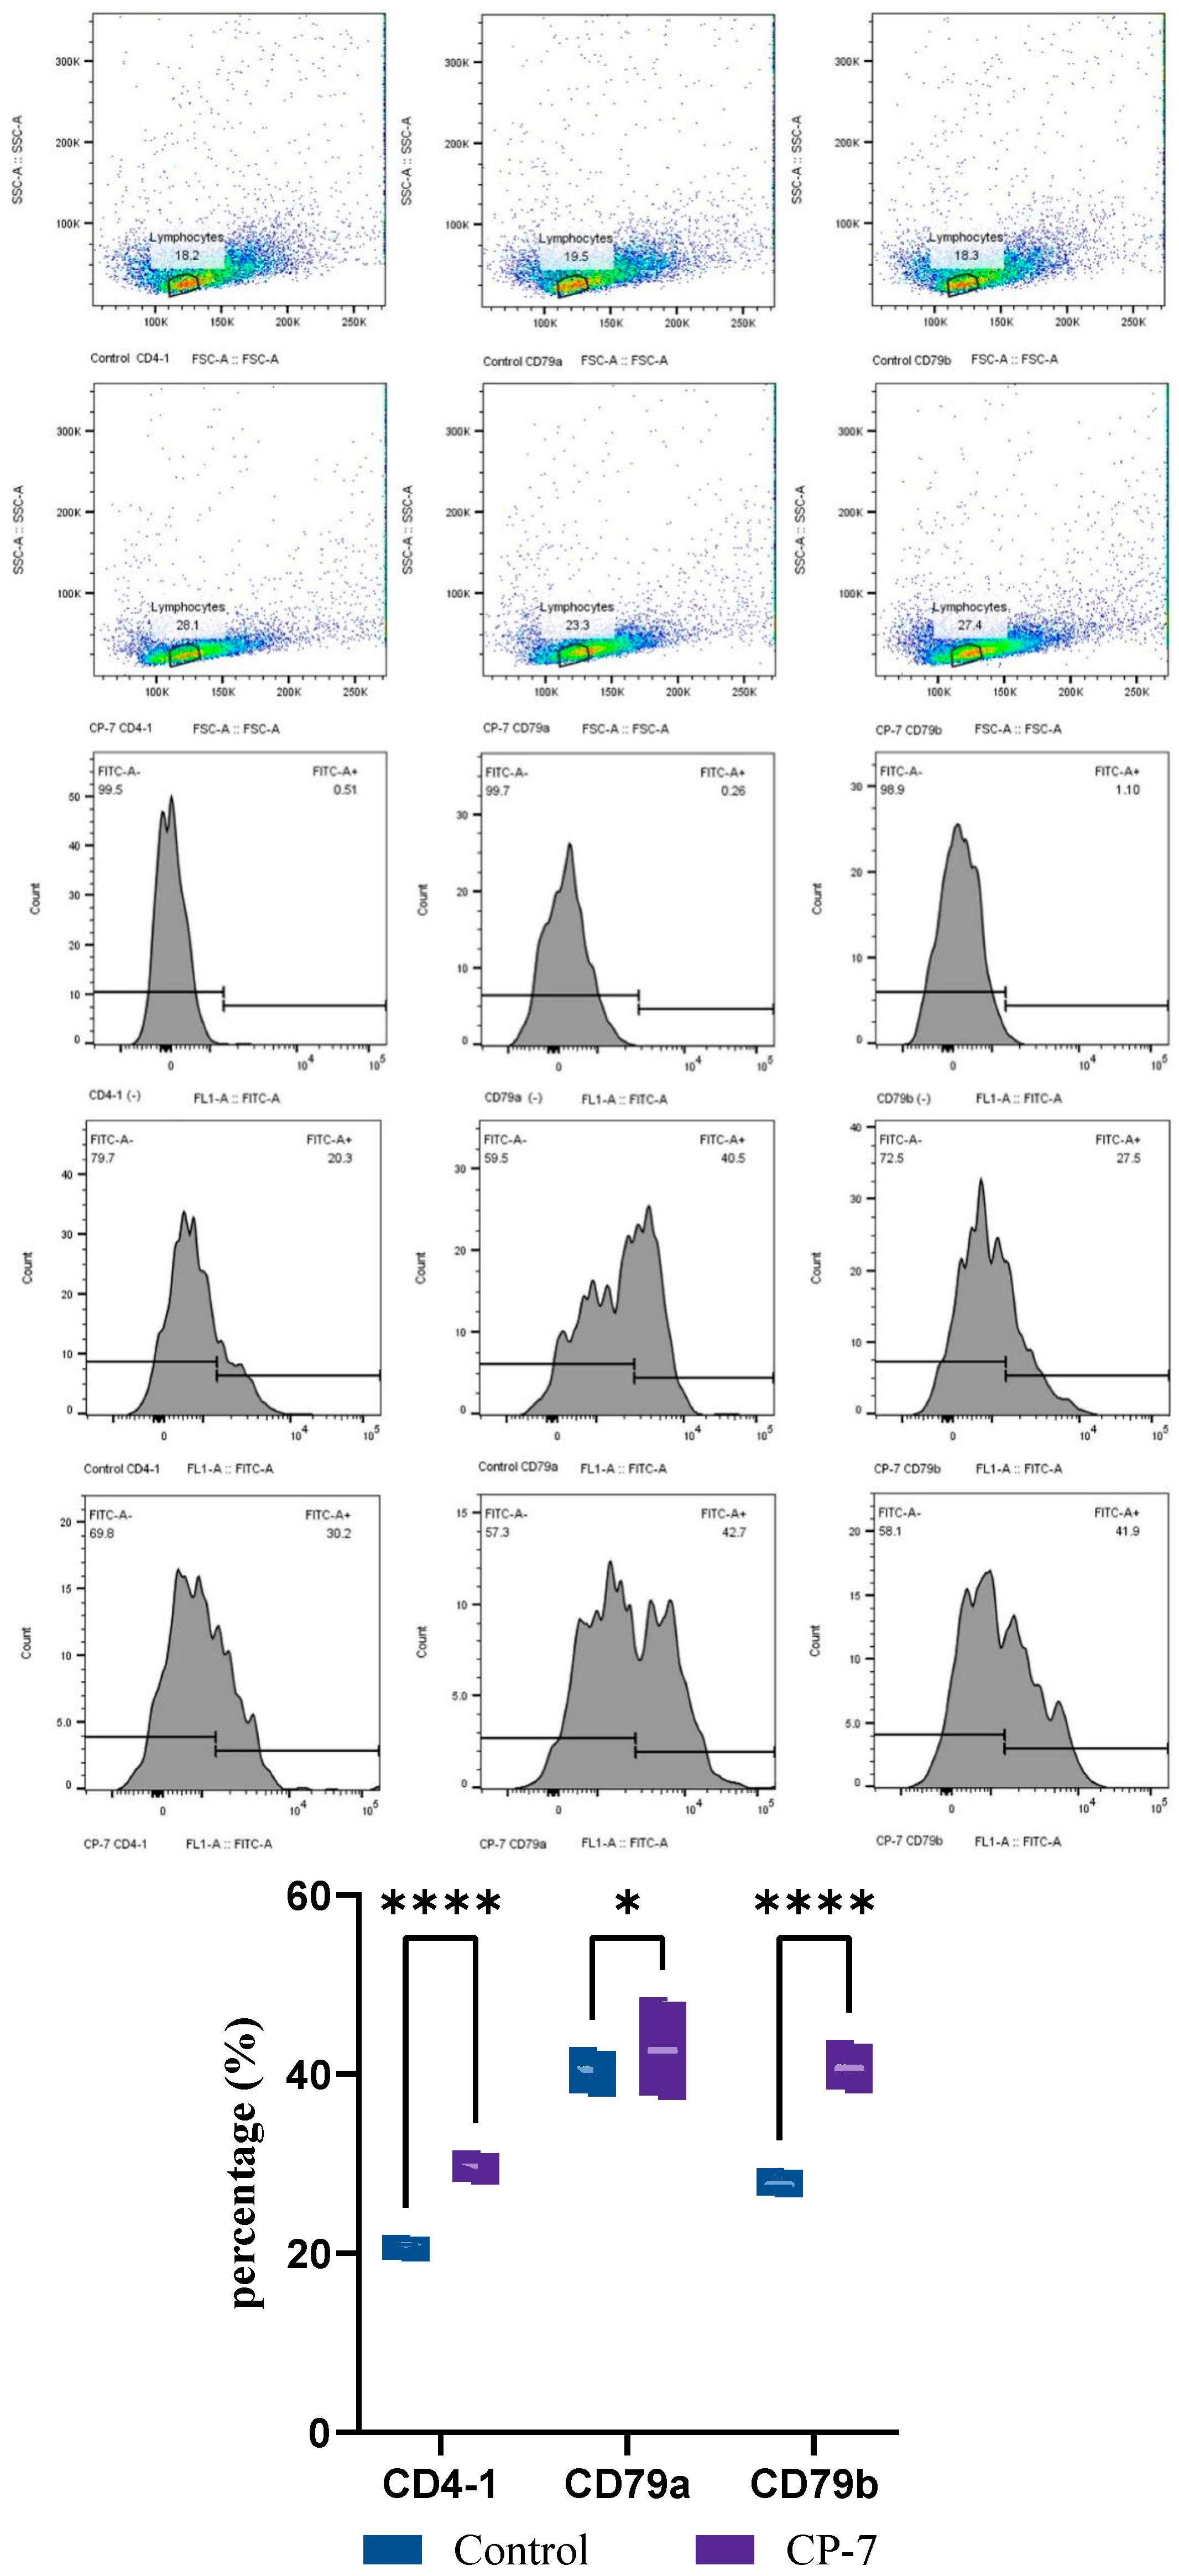
Flow cytometry was used to sort and count peripheral blood leukocytes of Sebastes schlegelii to further investigate the enhancement of adaptive immunity by carvacrol. After lymphocyte gating and doublet exclusion, sorting was performed via the FITC fluorescence channel, and the results are shown in Figure 8. As shown in the figure, the percentages of CD4-1+ T cells, CD79a+ B cells, and CD79b+ B cells in peripheral blood leukocytes of Sebastes schlegelii in the CP-7 group were significantly higher than those in the Control group.

4. Discussion

In the prophylactic part of this study, fish were challenged via the injection of V. harveyi, which better evaluates the host response to more acute toxic stress compared with immersion challenge after drug prophylaxis. Meanwhile, the injection model ensures a standardized and controllable bacterial dose, allowing for accurate assessment of host resistance and mortality. In contrast, the therapeutic group was challenged using an immersion model, which simulates the natural infection route in aquatic environments and is more consistent with actual aquaculture conditions. The combined use of these two models enables a comprehensive and reliable evaluation of disease resistance, rendering the experimental results more rigorous and robust.
As shown in the survival rate results, feeding with carvacrol increased the survival rate of S. schlegelii after immersion infection with V. harveyi. Histopathological tissue sections indicated that treating with carvacrol after V. harveyi infection could effectively alleviate phenomena such as aggregation of intestinal inflammatory cells, atrophy and shedding of intestinal villi, hemorrhage of intestinal tissue, and pyknosis of intestinal cell nuclei. These experimental results demonstrated that carvacrol can assist S. schlegelii in resisting the infection of V. harveyi.
NF-κB initiates and regulates the innate immune response to infection by modulating the expression of cytokines [30]. Existing studies have clearly demonstrated that IL-15 can maintain the homeostatic proliferation of memory CD8+ T cells and the persistence of CD8+ memory T cells. Moreover, it can also sustain the proliferative capacity of T cells and NK cells in vertebrates via the STAT5 signaling pathway [31,32]. The interleukin-12b (IL-12b) gene encodes the p40 chain of IL-12 [33]. Recent genomic research has identified IL12b as a susceptibility locus for inflammatory bowel disease (IBD) [34]. The findings of this study show that carvacrol intervention modifies the intestinal expression levels of NF-κB, IL-15 and IL-12b in experimental fish challenged with V. harveyi, suggesting that carvacrol might exert a regulatory influence on the host inflammatory response.
The results of enzyme activity analysis showed that both V. harveyi and carvacrol could influence the activities of ACP and AKP in the intestine of S. schlegelii, whereas neither treatment significantly affected the activities of SOD and CAT, nor MDA content. This finding suggests that the protective effect of carvacrol against V. harveyi stress is mediated via a non-oxidative defense mode.
The results obtained through conventional DNA extraction and sequencing encompass viable, dead, and dormant microbes in the intestine, making this approach suitable for profiling the species composition and relative proportions of intestinal microorganisms. In contrast, the reverse transcription method involves isolating labile intestinal RNA and reverse-transcribing it into complementary DNA (cDNA) before sequencing. This strategy solely reflects the composition of metabolically active intestinal microbes, thus facilitating the analysis of the activity status and functional potential of the intestinal microbial community. Analysis revealed that Vibrio was the microbial genus with significant differences in the intestine of experimental fish among groups as determined by both methods. The abundance of Vibrio in the challenged groups (HI, Control-PI2) measured by the two methods was significantly higher than those in the Control-P and Control-T groups, suggesting that both a 5-day immersion challenge with V. harveyi and a 2-day injection challenge significantly increased the intestinal Vibrio abundance of S. schlegelii. In the prevention section, the relative abundance of Vibrio in the CP-I2 group was substantially lower than that in the Control-PI2 group. In the treatment section, the results of the conventional method demonstrated that the Vibrio abundance in the CT-4 and CT-7 groups was significantly lower than that in the HI; the reverse transcription method showed that the Vibrio abundance in the CT-7 group was significantly lower than that in the HI group. Consistent results from the two relative quantification methods for pathogenic bacteria demonstrated that carvacrol could effectively inhibit the proliferation of Vibrio in the intestine of Sebastes schlegelii and improve host resistance against pathogenic bacterial invasion.
Regarding the effect on immunity, the administration of carvacrol significantly increased the proportion of CD4-1+ T cells and CD79a/CD79b+ B cells in visceral tissues of experimental fish. As key components of the immune system, CD4+ T cells play a central role in coordinating adaptive immune responses [35,36]. CD79 molecules are specific to B cells and are expressed during most developmental stages. Encoded by the CD79a and CD79b genes, they form a heterodimeric signaling unit within the B-cell receptor complex, responsible for transmitting signals for B-cell activation, proliferation, and differentiation [37,38]. The proportions of helper T cells and B lymphocytes in the total cell population can be determined via the specific binding of CD4-1, CD79a, and CD79b antibodies to cell surface antigens, which further reflects the activation of cellular and humoral immunity in the organism. Immunohistochemical (IHC) results showed that in fish receiving 7 days of carvacrol prophylaxis, the percentage of CD4-1+ T cells was significantly elevated in all detected tissues except the spleen, where no significant difference was observed compared with the control group. The percentages of CD79a/CD79b+ B cells were significantly increased in the liver, spleen, and head kidney of all treatment groups, and the positive cell trends detected by CD79a and CD79b were consistent. Flow cytometric analysis of peripheral blood showed that carvacrol significantly increased the proportions of CD4-1+ T cells and CD79a/CD79b+ B cells of the experimental fish. With prophylactic administration of carvacrol, the mean percentage of CD4-1+ T cells in peripheral blood increased from 20.77% to 29.73%; the proportion of CD79a+ B cells increased from 40.37% to 42.83%; the proportion of CD79b+ B cells increased from 27.93% to 40.87%. In conclusion, dietary administration of 500 mg/kg carvacrol can activate the proportion of T cells and B cells in experimental fish, thereby enhancing the efficiency of cellular and humoral immune responses against pathogenic stress.

5. Conclusions

In this study, S. schlegelii was selected as the experimental subject to thoroughly explore the preventive and immune-enhancing effects of carvacrol on uninfected juvenile S. schlegelii, as well as its therapeutic effect following pathogen infection. The results demonstrated that the administration of carvacrol could enhance the resistance of S. schlegelii to V. harveyi stress in farming environments, consequently improving the survival rates. This enhancement was accomplished through multiple mechanisms, including the improvement of intestinal histological morphology, the regulation of the expression of inflammation-related gene expression and phosphatase activity, the reconstruction of the intestinal microbial community, the reduction in Vibrio abundance, and the enhancement of the adaptive immunity, as well as increases in the proportions of CD4-1+ T cells and CD79a/CD79b+ B cells in key immune organs and peripheral blood. Collectively, these findings offer empirical data to support the healthy cultivation of S. schlegelii and promote the subsequent screening of alternative agents to antibiotic alternatives.

Author Contributions

T.W.: Data curation, Validation. Formal analysis, Methodology, Writing—original draft. Y.Y.: Investigation, Methodology, Software. C.W.: Investigation, Validation. Y.W.: Funding acquisition, Methodology, Formal analysis. Z.Z. (Zhiqi Zhang): Methodology, Formal analysis, Software. X.R.: Funding acquisition, Formal analysis. M.L.: Formal analysis, Methodology. K.H.: Formal analysis, Methodology. Z.Z. (Zheng Zhang): Conceptualization, Writing—review & editing, Methodology, Software, Funding acquisition. All authors have read and agreed to the published version of the manuscript.

Funding

This work was supported by the National Key Research and Development Program [grant numbers 2023YFD2400704], the Key Research and Development Program of Guangxi Province [grant number GUIKENONG-AB2506910047], the Central Public-Interest Scientific Institution Basal Research Fund [grant number 20603022025012 and 2023TD29], and the Hebei High-Level Talent Program [2023HBQZYCSB019].

Institutional Review Board Statement

The research in this manuscript has been conducted under the oversight of the Institutional Animal Care and Use Committee (IACUC) (approval code: YSFRI-2024059 and approval date: 27 April 2024).

Data Availability Statement

The original contributions presented in this study are included in the article. Further inquiries can be directed to the corresponding author.

Conflicts of Interest

Author Chunyuan Wang was employed by the company Huanghua Jinhui Aquaculture Development Co., Ltd. The remaining authors declare that the research was conducted in the absence of any commercial or financial relationships that could be construed as a potential conflict of interest.

References

  1. van Gelderen, T.A.; Debnath, P.; Joly, S.; Bertomeu, E.; Duncan, N.; Furones, D.; Ribas, L. Gonadal miRNomes and transcriptomes in infected fish reveal sexually dimorphic patterns of the immune response. Funct. Integr. Genom. 2025, 25, 29. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  2. Bloomfield, S.J.; Palau, R.; Janecko, N.; Baker-Austin, C.; Mather, A.E. Association of antimicrobial resistant Vibrio and species pathogenic to humans with aquacultured seafood. Food Microbiol. 2025, 132, 104819. [Google Scholar] [CrossRef] [Scilit]
  3. Zhang, B.Z.; Qiu, Y.L.; Shi, C.X.; Zhang, J. Development of Multiple Real-Time Fluorescent Quantitative PCR for Vibrio Pathogen Detection in Aquaculture. Vet. Sci. 2025, 12, 327. [Google Scholar] [CrossRef] [Scilit]
  4. Manchanayake, T.; Mohamad, A.; Amir-Danial, Z.; Abu Nor, N.; Yong-Kit, C.; Nazarudin, M.F.; Nor, R.M.; Hasnan, Q.; Zamri-Saad, M.; Amal, M.N.A.; et al. Oral adjuvanted Vibrio vaccine enhances antibody production and lysozyme activity in the serum and mucus of marine-cultured red hybrid tilapia (Oreochromis sp.) against V. harveyi and V. alginolyticus. Fish Shellfish Immunol. 2025, 165, 110503. [Google Scholar] [CrossRef] [Scilit]
  5. Choi, J.H.; Won, K.M.; Sohn, S.B.; Park, H.J.; Byun, S.G.; Lee, B.I.; Lee, J.H.; Kim, Y.C.; Park, S.I. Pathogenicity of Vibrio harveyi to black rockfish, Sebastes schlegeli. J. Fish Pathol. 2007, 20, 99–108. [Google Scholar]
  6. Strem, R.; Meiri-Ashkenazi, I.; Segal, N.a.; Ehrlich, R.; Shashar, N.; Sharon, G. Evaluation of Flathead Grey Mullets (Mugil cephalus) Immunization and Long-Term Protection against Vibrio harveyi Infection Using Three Different Vaccine Preparations. Int. J. Mol. Sci. 2023, 24, 8277. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  7. Wan, X.; Da, F.; Lin, G.; Huang, Y.; Cai, S.; Jian, J. Transcriptome Analysis of the Cultured Hybrid Grouper (♀Epinephelus fuscoguttatus × ♂E. lanceolatus) Immunized with Vibrio harveyi formalin-killed cells vaccine (FKC) combined with chitosan oligosaccharide. Isr. J. Aquac.-Bamidgeh 2023, 75, 1–9. [Google Scholar] [CrossRef] [Scilit]
  8. Yang, X.; Cheng, Y.; Zhao, Y.; Zhu, H.; Zhang, Y.; Zhao, Y.; Liu, X. Comparative transcriptome analysis reveals immunoregulation mechanism in the spleen of large yellow croaker (Larimichthys crocea) in response to Vibrio harveyi infection. Aquac. Rep. 2023, 31, 101657. [Google Scholar] [CrossRef] [Scilit]
  9. Milijasevic, M.; Veskovic-Moracanin, S.; Milijasevic, J.B.; Petrovic, J.; Nastasijevic, I. Antimicrobial Resistance in Aquaculture: Risk Mitigation Within One Health Context. Preprints 2024. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  10. Ma, P.; Chen, Y.; Shao, N.; Zhang, J.; Wu, Y.; Liu, R. Synergistic Combination of Biodegradable Peptide Polymer and Curcumin as Promising Antibiotic Substitution in Aquaculture to Alleviate the Global Challenge of Antimicrobial Resistance. Chin. J. Chem. 2022, 40, 2947–2955. [Google Scholar] [CrossRef] [Scilit]
  11. Pan, T.; Yan, M. The screening of traditional Chinese herbs on nonspecific immune response and protection of Pacific white shrimp (Litopenaeus vannamei) from Vibrio harveyi infection. Aquac. Int. 2020, 28, 767–776. [Google Scholar] [CrossRef] [Scilit]
  12. Wu, Q.; Jiang, Y.; Chen, E.; Mu, C.; Waiho, K. Chinese gallnut (Galla chinensis) against Vibrio parahaemolyticus: In vitro activity and the use of medicated bath method to treat infected mud crab Scylla paramamosain. Aquaculture 2021, 539, 736632. [Google Scholar] [CrossRef] [Scilit]
  13. Bhat, R.A.H.; Khangembam, V.C.C.; Pant, V.; Tandel, R.S.; Pandey, P.K.; Thakuria, D. Antibacterial Potential of a De-Novo Designed Peptide Against Bacterial Fish Pathogens. Int. J. Pept. Res. Ther. 2023, 29, 85. [Google Scholar] [CrossRef] [Scilit]
  14. Prazdnova, E.; Zaikina, A.; Neurov, A.; Mazanko, M.; Ranjan, A.; Rudoy, D. Bacillibactin, a Potential Bacillus-Based Antibacterial Non-Ribosomal Peptide: In Silico Studies for Targeting Common Fish Pathogens. Int. J. Mol. Sci. 2025, 26, 5811. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  15. Imtiaz, N.; Anwar, Z.; Waiho, K.; Shi, C.; Mu, C.; Wang, C.; Wu, Q. A review on aquaculture adaptation for fish treatment from antibiotic to vaccine prophylaxis. Aquac. Int. 2024, 32, 2643–2668. [Google Scholar] [CrossRef] [Scilit]
  16. Tayyab, M.; Islam, W.; Waqas, W.; Zhang, Y. Probiotic-Vaccine Synergy in Fish Aquaculture: Exploring Microbiome-Immune Interactions for Enhanced Vaccine Efficacy. Biology 2025, 14, 629. [Google Scholar] [CrossRef] [Scilit]
  17. Wang, Q.; Huang, J.; Li, Y.; Wu, S.; Zhao, L.; Pan, Y.; Kang, Y.; Liu, Z. Chinese herbal medicines mixture improved antioxidant enzymes, immunity and disease resistance to infectious hematopoietic necrosis virus infection in rainbow trout (Oncorhynchus mykiss). Aquac. Int. 2024, 32, 3217–3232. [Google Scholar] [CrossRef] [Scilit]
  18. Zhu, Z.-X.; Yao, Y.-Y.; Ai, C.-H.; Yang, G.; Liang, X.-Y.; Liu, T.-D.; He, M.-L.; Xia, J.-H. Dietary supplementation of Patchouli oil increases the resistance against Streptococcus agalactiae infection in GIFT tilapia as revealed by transcriptome and 16s amplicon profiling. Aquac. Rep. 2023, 33, 101754. [Google Scholar] [CrossRef] [Scilit]
  19. Xu, M.; Li, H.; Wu, X.; Dai, L.; Yang, R.; Zhang, Q.; Zhang, Z.; Lei, L.; Zhang, F. Inhibitory effect of arctigenin on reovirus infection in grass carp. Aquaculture 2024, 593, 741355. [Google Scholar] [CrossRef] [Scilit]
  20. Yu, B.; Sun, Z.; Li, X.C.; Qv, A.; Sohail, M.; Li, Y.L.; Xu, H.; Xiang, P. Research Progress of Novel Drug Delivery Systems of Chinese Medicine Monomers based on Natural Silk Fibroin: A Mini-Review. Curr. Drug Deliv. 2023, 20, 211–222. [Google Scholar] [CrossRef] [Scilit]
  21. Alagawany, M.; Farag, M.R.; Salah, A.S.; Mahmoud, M.A. The role of oregano herb and its derivatives as immunomodulators in fish. Rev. Aquac. 2020, 12, 2481–2492. [Google Scholar] [CrossRef] [Scilit]
  22. Hirose, S.; Horiyama, S.; Morikami, A.; Fujiwara, K.; Tsukagoshi, H. Eugenol and basil essential oil as priming agents for enhancing Arabidopsis immune response. Biosci. Biotechnol. Biochem. 2024, 89, 41–50. [Google Scholar] [CrossRef] [Scilit]
  23. Deng, H.; Deng, Y.; Song, T.; Pang, L.; Zhu, S.; Ren, Z.; Guo, H.; Xu, Z.; Zhu, L.; Geng, Y.; et al. Evaluation of the activity and mechanisms of oregano essential oil against PRV in vivo and in vitro. Microb. Pathog. 2024, 194, 106791. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  24. Zhou, F.; Ji, B.P.; Zhang, H.; Jiang, H.; Yang, Z.W.; Li, J.J.; Li, J.H.; Yan, W.J. The antibacterial effect of cinnamaldehyde, thymol, carvacrol and their combinations against the foodborne pathogen Salmonella typhimurium. J. Food Saf. 2007, 27, 124–133. [Google Scholar] [CrossRef] [Scilit]
  25. Das, S.; Chourashi, R.; Mukherjee, P.; Kundu, S.; Koley, H.; Dutta, M.; Mukhopadhyay, A.K.; Okamoto, K.; Chatterjee, N.S. Inhibition of growth and virulence of Vibrio cholerae by carvacrol, an essential oil component of Origanum spp. J. Appl. Microbiol. 2021, 131, 1147–1161. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  26. Coelho, J.D.; Rosa, K.V.; Rocha, J.S.; Ramirez, N.C.B.; Maraschin, M.; Vieira, F.D. In Vitro Antimicrobial Activity of Carvacrol Against Shrimp Pathogens and Its Use as Feed Additive for the Pacific White Shrimp. Bol. Inst. Pesca 2021, 47, e645. [Google Scholar] [CrossRef] [Scilit]
  27. Rossi, B.; Esteban, M.A.; Garcia-Beltran, J.M.; Giovagnoni, G.; Cuesta, A.; Piva, A.; Grilli, E. Antimicrobial Power of Organic Acids and Nature-Identical Compounds against Two Vibrio spp.: An In Vitro Study. Microorganisms 2021, 9, 966. [Google Scholar] [CrossRef] [Scilit]
  28. Wang, J.; Mai, K.; Ai, Q. Conventional Soybean Meal as Fishmeal Alternative in Diets of Japanese Seabass (Lateolabrax japonicus): Effects of Functional Additives on Growth, Immunity, Antioxidant Capacity and Disease Resistance. Antioxidants 2022, 11, 951. [Google Scholar] [CrossRef] [Scilit]
  29. Ahmadifar, E.; Mansour, M.R.; Amirkolaie, A.K.; Rayeni, M.F. Growth efficiency, survival and haematological changes in great sturgeon (Huso huso Linnaeus, 1758) juveniles fed diets supplemented with different levels of thymol-carvacrol. Anim. Feed Sci. Technol. 2014, 198, 304–308. [Google Scholar] [CrossRef] [Scilit]
  30. Pittet, L.A.; Quinton, L.J.; Yamamoto, K.; Robson, B.E.; Ferrari, J.D.; Algül, H.; Schmid, R.M.; Mizgerd, J.P. Earliest Innate Immune Responses Require Macrophage RelA during Pneumococcal Pneumonia. Am. J. Respir. Cell Mol. Biol. 2011, 45, 573–581. [Google Scholar] [CrossRef] [Scilit]
  31. Drake, A.; Kaur, M.; Iliopoulou, B.P.; Phennicie, R.; Hanson, A.; Chen, J.Z. Interleukins 7 and 15 Maintain Human T Cell Proliferative Capacity through STAT5 Signaling. PLoS ONE 2016, 11, e0166280. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  32. Clark, S.E.; Burrack, K.S.; Jameson, S.C.; Hamilton, S.E.; Lenz, L.L. NK Cell IL-10 Production Requires IL-15 and IL-10 Driven STAT3 Activation. Front. Immunol. 2019, 10, 2087. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  33. Xu, Z.; Pei, L.; Zhang, F.; Hu, X.; Gui, Y.; Wang, L.; Wu, B. A functional variant in IL12B promoter modulates its expression and associates with increased risk of allergic asthma. Genes Immun. 2013, 14, 238–243. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  34. Márquez, A.; Mendoza, J.L.; Toxonera, C.; Díaz-Rubio, M.; de la Concha, E.G.; Urcelay, E.; Martínez, A. IL23R and IL12B polymorphisms in Spanish IBD patients: No evidence of interaction. Inflamm. Bowel Dis. 2008, 14, 1192–1196. [Google Scholar] [CrossRef] [Scilit]
  35. Zhu, X.L.; Zhu, J.F. CD4 T Helper Cell Subsets and Related Human Immunological Disorders. Int. J. Mol. Sci. 2020, 21, 8011. [Google Scholar] [CrossRef] [Scilit]
  36. Maisey, K.; Montero, R.; Corripio-Miyar, Y.; Toro-Ascuy, D.; Valenzuela, B.; Reyes-Cerpa, S.; Sandino, A.M.; Zou, J.; Wang, T.H.; Secombes, C.J.; et al. Isolation and Characterization of Salmonid CD4+ T Cells. J. Immunol. 2016, 196, 4150–4163. [Google Scholar] [CrossRef] [Scilit]
  37. Huang, X.G.; Takata, K.; Sato, Y.; Tanaka, T.; Ichimura, K.; Tamura, M.; Oka, T.; Yoshino, T. Downregulation of the B-cell receptor signaling component CD79b in plasma cell myeloma: A possible post transcriptional regulation. Pathol. Int. 2011, 61, 122–129. [Google Scholar] [CrossRef] [Scilit]
  38. Huse, K.; Bai, B.Y.; Hilden, V.I.; Bollum, L.K.; Våtsveen, T.K.; Munthe, L.A.; Smeland, E.B.; Irish, J.M.; Wälchli, S.; Myklebust, J.H. Mechanism of CD79A and CD79B Support for IgM plus B Cell Fitness through B Cell Receptor Surface Expression. J. Immunol. 2022, 209, 2042–2053. [Google Scholar] [CrossRef] [Scilit]
Figure 1. Experimental fish sampling flow chart.
Fishes 11 00273 g001
Figure 2. Apparent symptoms of experimental fish in the 2-day intramuscular injection challenge group (Control-PI2) and the 5-day Vibrio harveyi immersion challenge group (HI). (A,B): External appearance images of experimental fish in the Control-PI2 group and HI. (C,D): Local symptom images of experimental fish in the Control-PI2 group and HI group. (E,F): Anatomical images of experimental fish in the Control-PI2 group and HI group.
Fishes 11 00273 g002
Figure 3. Survival rates of experimental fish in different groups. Contro-P: Control group in the prevention trial. CP: Carvacrol prevention group. Control-PI2: Group with 7-day blank diet feeding followed by 2-day V. harveyi injection challenge. CP-I2: Group with 7-day feeding of 500 mg/kg carvacrol-supplemented diet followed by 2-day V. harveyi injection challenge. Control-T: Control group in the treatment trial. HI: Group subjected to 5-day V. harveyi immersion challenge. CT: Carvacrol-treated therapeutic group.
Fishes 11 00273 g003
Figure 4. Intestinal pathological sections of experimental fish in each group (20× magnification). (A): Intestinal pathological section of fish in the control group of the prevention trial (Control-P). (B): Intestinal pathological section of fish in the carvacrol prevention 7-day group (CP-7). (C): Intestinal pathological section of fish in the group injected with V. harveyi for 2 days after 7 days of feeding with a blank diet (Control-PI2). (D): Intestinal pathological section of fish in the group injected with V. harveyi for 2 days after 7-day feeding with carvacrol-supplemented diet (CP-I2). (E): Intestinal pathological section of fish in the control group of the treatment trial (Control-T). (F): Intestinal pathological section of fish in the group immersed with V. harveyi for 5 days (HI). (G): Intestinal pathological section of fish in the carvacrol treatment 4-day group after challenge (CT-4). (H): Intestinal pathological section of fish in the carvacrol treatment 7-day group after challenge (CT-7). Scale bar = 0.050 mm.
Fishes 11 00273 g004
Figure 5. (A,B): Bar charts depicting the relative abundance of intestinal microbiota in the experimental fish of each group. (C,D): Differences in Vibrio abundance between the groups, detected using the conventional method and reverse-transcription method, respectively. * indicates p < 0.05, ** indicates p < 0.01, *** indicates p < 0.001, and no symbol means no significant difference.
Fishes 11 00273 g005
Figure 6. Expression levels of inflammation-related genes and hepatic enzyme activities in each group. (A): Expression levels of inflammation-related genes in the prevention phase. (B): Expression levels of inflammation-related genes in the treatment section groups. (C): Hepatic enzyme activities of experimental fish from different groups in the prevention phase. (D): Hepatic enzyme activities of experimental fish from different groups in the treatment phase. * indicates p < 0.05, ** indicates p < 0.01, *** indicates p < 0.001, **** indicates p < 0.0001, and no symbol means no significant difference.
Fishes 11 00273 g006
Figure 7. Changes in the proportions of CD4-1+ T cells, CD79a+ B cells and CD79b+ B cells in various tissues for the group with 7-day carvacrol prevention. *** indicates p < 0.001, **** indicates p < 0.0001, and no symbol means no significant difference.
Fishes 11 00273 g007
Figure 8. Changes in CD4-1+ T cells, CD79a+ B cells and CD79b+ B cells in peripheral blood of experimental fish with 7-day carvacrol prevention. * indicates p < 0.05, **** indicates p < 0.0001, and no symbol means no significant difference.
Fishes 11 00273 g008
Table 1. Target genes and their primers for qPCR.
Target GenePrimerNucleotide Sequence 5′-3′
RPL-17RPL17-FAGGCGACGCACCTACCG
RPL17-RCCTCTGGTTTGGGGACGA
NFκB/RelANFκB/RelA-FTGTCGTAGATGGGGTTGGA
NFκB/RelA-RAGGAGCTGGGGAAGGTGAT
IL-12bIL-12b-FCTCTGGCATCCTTATCAGTTCA
IL-12b-RGTCTTGGTTGCTGGCGTAG
IL-15IL-15-FCGCCTACAATACAACTAAAGAGC
IL-15-RAGATGACGGAGCATACAGCA
Table 2. Intestinal abundance of Vibrio in the experimental fish from each treatment group.
GroupVibrio Abundance Determined by DNA Extraction Method (%)Vibrio Abundance Determined by RNA Extraction and Reverse Transcription (%)
Control-P<0.0642.08
CP-70.3238.25
Control-PI246.5992.54
CP-I216.884.59
Control-T0.0631.12
HI48.5578.27
CT-40.8480.14
CT-70.9529.71
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.