Article

Genome-Wide Identification of the U-Box Gene Family and Expression Analysis in Response to Salt Stress in Melon


1
College of Horticulture, Northeast Agricultural University, Harbin 150030, China
2
Key Laboratory of Biology and Genetic Improvement of Horticulture Crops (Northeast Region), Ministry of Agriculture and Rural Affairs, College of Horticulture, Northeast Agricultural University, Harbin 150030, China
*
Authors to whom correspondence should be addressed.
†
These authors contributed equally to this work.
Horticulturae 2026, 12(10), 1215; https://doi.org/10.3390/horticulturae12101215
Submission received: 10 August 2026 / Revised: 17 September 2026 / Accepted: 24 September 2026 / Published: 26 September 2026
(This article belongs to the Section Biotic and Abiotic Stress)

Abstract

The U-box proteins (PUBs), as a prominent family of E3 ubiquitin ligases, have been reported to participate in diverse physiological processes, such as plant development, growth regulation, and adaptation to abiotic and biotic stresses. Nevertheless, a comprehensive genome-wide survey and functional investigation of the U-box family in melon remain limited. In this study, a total of 50 CmPUB genes harboring the U-box domain were identified and distributed across the 12 melon chromosomes. Phylogenetic analysis among melon, cucumber, tomato and Arabidopsis divided the 50 CmPUBs into six subfamilies. CmPUB37/48/49 are orthologous to salt stress-responsive AtPUB18/19 in Arabidopsis. Intraspecies collinearity analyses detected 11 homologous gene pairs within the CmPUB family and 15 to 67 collinear genes among five other species, respectively, based on the interspecies collinearity analyses. Promoter analysis revealed that CmPUBs had diverse and abundant cis-acting regulatory elements involved in light signal transduction, phytohormone regulation, and stress responses, as well as plant development. Transcriptome analysis of the CmPUBs in melon under salt stress revealed that most CmPUBs exhibited temporally differentiated expression patterns, with some genes being rapidly induced at the early stage of stress and continuously upregulated at the late stage. Physiological measurements under salt stress indicated that leaves were the primary tissue responding to salt-induced oxidative damage, and that the salt-tolerant line M4-116 alleviated this damage by maintaining higher superoxide dismutase (SOD) and catalase (CAT) activities and lower malondialdehyde (MDA) accumulation than the salt-sensitive line M4-75. Quantitative real-time PCR (qRT-PCR) was conducted using leaf tissues harvested at multiple time intervals. The expression patterns were compared between salt-tolerant and salt-sensitive cultivars, revealing that transcript levels were markedly elevated in the salt-tolerant cultivar under salt stress conditions. In conclusion, this study provides a foundation for further functional studies of U-box genes and offers new insights into stress responses in melon.

1. Introduction

Melon (Cucumis melo L.), belonging to the Cucurbitaceae family, represents an important horticultural crop worldwide due to its desirable fruit characteristics and high economic value [1]. In major melon-cultivating areas under protected cultivation across China, however, salt stress caused primarily by secondary soil salinization has grown increasingly common. It severely limits plant growth and impairs fruit quality, and has become a core bottleneck restricting the stable development of the whole industry [2]. An increasing body of evidence indicates that protein ubiquitination, as a key post-translational regulatory mechanism, can regulate plant tolerance to salt stress by modulating ion homeostasis, stress signal transduction, and protein quality control [3].
The ubiquitin-26S proteasome system (UPS) in eukaryotes handles post-translational modification and specific degradation of proteins, playing a crucial role in controlling the cell cycle, signal transduction, and stress responses, among other biological processes. This modification is mediated by a sequential ubiquitination pathway that requires the coordinated action of three key enzymes: ubiquitin-activating enzyme E1, ubiquitin-conjugating enzyme E2, and ubiquitin ligase E3 [4]. Within the ubiquitin-mediated degradation pathway, E3 ligases are responsible for recognizing specific target proteins and thereby regulating substrate selection. Notably, plant genomes typically contain a substantially larger repertoire of E3 ligase genes compared with those encoding E1 and E2 enzymes, suggesting that this enzyme group has evolved considerable functional complexity and plays essential roles in various plant processes [5,6]. E3 ubiquitin ligases, as essential components of the UPS, determine substrate recognition and specificity by facilitating the attachment of ubiquitin molecules to target proteins through interactions with E2 conjugating enzymes [7]. These ligases can finely regulate the stability, activity, and interactions of proteins by controlling their ubiquitination status, thereby maintaining intracellular protein homeostasis and eliminating misfolded or aggregated proteins [8]. Monomeric E3 ubiquitin ligases can be classified into three subtypes based on structural features and catalytic mechanisms: HECT-type, which is homologous to the C-terminus of E6-AP; RING-type, referring to Really Interesting New Gene; and RING-Between-RING (RBR) type [4,9]. The U-box domain represents an altered form of the RING finger motif and was first discovered in the yeast UFD2 protein [10]. Although the U-box domain adopts a structural conformation comparable to that of the RING domain, it does not possess the zinc-binding activity characteristic of RING motifs [11]. Instead, the stability of the U-box structure is primarily maintained through hydrogen bonding and hydrophobic interactions, representing a distinct structural feature that differentiates U-box-containing E3 ligases from conventional RING-type E3 ligases [12]. In plants, PUB proteins are defined by the presence of a conserved U-box domain, and several members of this family have been reported to function as monomeric E3 ligases [13]. Besides the U-box region, many PUB proteins harbor additional interaction-related domains, such as ARM repeats, kinase domains, and WD40 domains. These auxiliary domains contribute to substrate binding and protein interactions, which may underlie the diverse regulatory functions of PUB proteins [14,15].
Numerous studies have proven PUB proteins to be central regulators in growth regulation, innate immunity, phytohormone signal transduction, and abiotic stress adaptation [16,17,18,19,20,21]. In Arabidopsis, AtPUB11 inhibits the abscisic acid-regulated drought stress response by ubiquitinating and degrading receptor-like protein kinases LRR1 and KIN7 [22]; whereas AtPUB22 and AtPUB23 exert similar negative effects by degrading the ABA core receptor PYL9 [23]. In contrast, OsPUB67 can positively regulate plant drought tolerance by targeting the negative drought regulator OsRZFP34 [24]. The Arabidopsis E3 ubiquitin ligase AtPUB19 is strongly induced by salt stress and ABA, and collaborates with its homolog AtPUB18 to regulate ABA-mediated seed germination under salt stress [25]. In wheat, TaPUB15 is strongly upregulated by salt, drought and other abiotic stresses, and its overexpression significantly enhances salt tolerance [26]. AtPUB25 and AtPUB26 ubiquitinate and degrade MYB15, a negative regulator of cold signaling, thereby significantly enhancing cold tolerance [27]. Collectively, the PUB gene family is emerging as a core regulatory gene family for plant abiotic stress responses. Therefore, systematic identification and characterization of stress-responsive PUBs in melon are essential for the genetic improvement of stress-tolerant melon varieties.
To date, extensive studies in model and crop plants have identified varying numbers of PUB family members, ranging from 53 to 125 across the reported species. Representative PUB family sizes in Arabidopsis, rice, tobacco, eggplant, cucumber, tomato, barley, soybean, foxtail millet, and cabbage are summarized in Supplementary Table S1 [2,28,29,30,31,32,33,34,35]. The above research results have built a reliable research system for studies in comparative genomics and functional genomics. Nevertheless, comprehensive genome-level investigations of this gene family in melon remain insufficient. Here, we employed the newly released melon DHL92 reference genome (version 4.0) to conduct further analyses [36] to perform a genome-wide identification of CmPUBs, and subsequently analyzed their expression under salt stress. Overall, this study provides important theoretical support for the functional research of U-box genes in melon.

2. Materials and Methods

2.1. Identification of CmPUB Members

The genomic and protein datasets of melon DHL92 (version 4.0) were downloaded from the CuGenDBv2 portal (http://cucurbitgenomics.org/v2/, accessed on 22 April 2026). In addition, nucleotide and protein sequences corresponding to the Arabidopsis PUB family were obtained through the Arabidopsis Information Resource (http://www.arabidopsis.org/browse/genefamly/pub.jsp, accessed on 22 April 2026) and used as reference sequences for candidate identification.
A combination of homology-based and domain-based approaches was used to identify CmPUB genes. First, the Arabidopsis PUB protein sequences were used as queries for BLASTp (TBtools-II v2.303, China) searches against the melon protein dataset. Candidate proteins with an E-value <1 × 10⁻⁵ were retained. In parallel, the U-box domain profile (PF04564) was retrieved from the Pfam database [37] and used to construct a hidden Markov model (HMM). The melon proteome was subsequently searched using HMMER (http://hmmer.janelia.org/, accessed on 22 April 2026), with an E-value threshold of <1 × 10⁻⁵. Subsequently, the candidate sequences obtained through BLASTp and HMMER methods were compared, and the sequences common to both candidate sets were retained as the candidate sequences for CmPUB. Conserved domains of the resulting candidate proteins were further examined using the NCBI Conserved Domain Database (CDD; https://www.ncbi.nlm.nih.gov/cdd, accessed on 25 April 2026). Candidate proteins that lacked a complete U-box domain were removed. This procedure resulted in 50 non-redundant CmPUB proteins containing a complete U-box domain, which were designated CmPUB01 to CmPUB50.
The main physicochemical properties, namely molecular weight and isoelectric point (pI), were calculated using TBtools-II (v2.303, China) [38]. We used the WoLF PSORT online tool (URL: https://wolfpsort.hgc.jp/, last accessed on 25 April 2026) to complete the prediction of protein subcellular localization. The U-box family genes in melon are all named according to their positions on the chromosomes, with the designation CmPUB followed by a number (e.g., CmPUB01), where “Cm” represents Cucumis melo, “PUB” denotes the Plant U-box protein, and the following number indicates the order based on chromosomal position.

2.2. Gene Structure and Chromosomal Localization

Chromosomal location information for the 12 melon chromosomes was obtained through the CuGenDBv2 platform (http://cucurbitgenomics.org/v2/, accessed on 22 April 2026). We used the MEME online tool [39] to identify the conserved motifs of CmPUBs and analyzed the exon–intron structure with TBtools-II [38]. The conserved motifs were analyzed using MEME software (MEME Suite 5.5.8, USA), with the parameters set as follows: maximum number of motifs = 10, motif length range = 6 to 100 amino acid residues.

2.3. Phylogenetic Analysis and Protein Domain Analysis

PUB protein sequences from Arabidopsis thaliana, cucumber (Cucumis sativus), and tomato (Solanum lycopersicum) were obtained from previously published PUB family studies and the corresponding databases cited therein [28,31,32]. All PUB family members reported in these studies were included. Together with the 50 CmPUB proteins identified in this study, a total of 229 PUB protein sequences were used for phylogenetic analysis.
The amino acid sequences of CmPUB proteins were aligned with MEGA 11 [40], and a neighbor-joining (NJ) phylogenetic tree was subsequently constructed with 1000 bootstrap replicates to evaluate the branch reliability of the tree topology. The resulting phylogenetic tree was graphically displayed using the iTOL v6 web-based platform [41].

2.4. Promoter Analysis and Gene Ontology Annotation

The 2000 bp promoter regions upstream of 50 CmPUBs were extracted and analyzed through the PlantCARE database [42] to identify potential cis-regulatory elements. The predicted elements were subsequently displayed with TBtools-II [38].

2.5. Analysis of Collinearity and Duplication Events

Syntenic relationships within the melon genome were investigated using TBtools-II, and comparative collinearity analysis was further carried out between melon and five representative plant species, including Arabidopsis, cucumber, tomato, rice, and maize [38]. Genome annotation files were obtained from TAIR (https://www.arabidopsis.org/, accessed on 9 May 2026) and the Plants Ensembl database (https://plants.ensembl.org/index.html, accessed on 9 May 2026).

2.6. Protein Structure Analysis

Protein structures of the identified CmPUB family members were predicted using AlphaFold 3 (https://alphafoldserver.com/, accessed on 9 June 2026). The predicted three-dimensional models of 50 CmPUB proteins were generated using the AlphaFold Server based on their corresponding amino acid sequences under the default settings. The resulting structures were visualized and rendered using PyMOL (version 3.0, LLC). The pTM score was used as an overall confidence metric, and proteins with pTM ≥ 0.5 were selected for subsequent structural analyses. Prediction reliability was further assessed using residue-level pLDDT scores and predicted aligned error (PAE) plots. Regions with pLDDT scores >80 were considered to have high local prediction confidence, while PAE values were used to assess the confidence of relative positioning between structural regions or domains.

2.7. Plant Materials Salt Stress Treatment

The salt-sensitive cultivar M4-75 (Cucumis melo ssp. melo) and the salt-tolerant cultivar M4-116 (Cucumis melo ssp. melo) were selected for salt stress treatment and gene expression verification. The seeds were surface-disinfected using sodium hypochlorite solution for 10 min, followed by five washes with sterile distilled water. Afterward, the seeds were immersed in distilled water at room temperature for 6 h before being transferred to a hydroponic cultivation system. The plants were grown in a growth chamber with 12 h of light and 12 h of darkness, a temperature of 28 °C/22 °C (day/night), and 65% relative humidity.
At the three-true-leaf stage, plants were treated with 150 mM NaCl (Table S2), while water-treated plants were used as the untreated control. Roots, stems, and leaves were collected from both cultivars at 0, 6, 12, 24, and 48 h after NaCl treatment. For each biological replicate, one plant was used, and the second and third leaves were collected and pooled to obtain one composite leaf sample. Three biological replicates were included for each cultivar, treatment, and sampling time point. Physiological parameters, including SOD, CAT, and MDA, were measured in roots, stems, and leaves, whereas quantitative real-time PCR (qRT-PCR) analysis was performed using leaf samples only. All samples were immediately stored at −80 °C until further analysis.

2.8. Determination of Physiological Indicators

Under 150 mM sodium chloride conditions, root, stem, and leaf samples collected from the salt-tolerant cultivar M4-116 and the salt-sensitive cultivar M4-75 were tested for SOD and CAT activity as well as MDA content at 0, 6, 12, 24, and 48 h.
SOD activity was measured using a superoxide dismutase assay kit (Solarbio, Beijing, China) based on the nitroblue tetrazolium (NBT) photochemical reduction method. One unit of SOD activity is defined as the amount of enzyme needed to achieve a 50% inhibition of NBT photochemical reduction per gram of fresh weight (FW) tissue; the results are expressed as U/g FW. CAT activity was measured using a catalase assay kit (Solarbio, Beijing, China) based on the ultraviolet absorption principle. One unit of CAT activity was defined as the amount of enzyme that decomposes 1 μmol of H2O2 per gram of fresh weight tissue per minute, and the results were expressed as U/g FW. MDA content was detected using a malondialdehyde assay kit (Solarbio, Beijing, China) based on the thiobarbituric acid (TBA) colorimetric method. The results were expressed as nanomoles of MDA per gram of fresh weight tissue (nmol/g FW). All measurements for the above indicators were performed with three biological replicates.

2.9. Gene Expression Analysis

Transcriptome data from melon under salt stress were obtained from the NCBI BioProject PRJNA987131 [43]. The raw RNA-Seq data were processed using fastp to remove adapter sequences and low-quality bases, generating clean reads [44]. The clean reads were subsequently aligned to the melon reference genome using HISAT2, followed by transcript assembly and expression quantification using StringTie [45,46]. The resulting expression matrix was used to extract the expression profiles of the 50 identified CmPUB genes at different time points under salt stress. The expression patterns of all 50 CmPUB genes were visualized to characterize their temporal expression trends. No differential-expression analysis or differential-expression-based filtering was performed in this analysis.
Total RNA isolated from the collected tissue materials was prepared with the E.Z.N.A.® Plant RNA Kit (Omega Bio-tek, Norcross, GA, USA). First-strand cDNA synthesis was carried out using the PrimeScript™ FAST RT Kit (TaKaRa, Dalian, China). The transcript levels of CmPUBs were quantified based on the 2−∆∆Ct calculation method, using MELO3C023264 as the reference Actin gene [47,48]. The primer information is provided in Table S3.

2.10. Statistical Analysis

Raw data were organized in Excel 2024, while statistics and plotting were completed via Prism 10.0 (GraphPad Inc., Boston, MA, USA). Data were analyzed using descriptive statistics and analysis of variance (ANOVA). Homogeneity of variances was assessed before ANOVA. Because each group contained only three biological replicates (n = 3), formal assessment of normality was not considered sufficiently informative, and no normality test was used to infer normality from these data. When significant differences were detected by ANOVA, the least significant difference (LSD) test was used for multiple comparisons at p < 0.05.

3. Results

3.1. Characterization and Identification of CmPUBs in Melon

The PUB protein family in melon was systematically characterized through integrated genomic analyses. First, we used the protein sequences of Arabidopsis U-box proteins as a reference to perform a BLASTp search against the melon DHL92 genome (version 4.0), and identified 706 potential PUB gene candidates. Secondly, using the HMM profile of the U-box domain (PF04564) and the HMMER search method, 58 candidate PUB genes were identified from the whole melon genome. Thirdly, the two candidate sets were then compared, and their intersection yielded 51 putative CmPUB candidates. Finally, these candidates were subsequently examined using the NCBI Conserved Domain Database (CDD) to confirm the presence and integrity of the U-box domain. One candidate was excluded because it did not contain a complete U-box domain, resulting in a final set of 50 non-redundant CmPUB genes. These genes were designated CmPUB01–CmPUB50 according to their chromosomal positions. The complete identification and screening procedure is summarized in a PRISMA-style flowchart (Figure S1).
The physicochemical characteristics of CmPUB proteins were systematically examined, including protein length, predicted molecular mass, theoretical pI values, and corresponding gene IDs (Table S4). The 50 CmPUB proteins exhibited significant differences in both sequence and physicochemical properties. The encoded proteins showed considerable variation in size, with amino acid numbers ranging from 365 residues in CmPUB28 to 1488 residues in CmPUB13. Their predicted molecular masses ranged between 34,330.89 Da and 165,576.47 Da. The instability index ranged from 34.98 to 58.28, while the aliphatic index ranged from 66.6 to 118.59. Among them, CmPUB14 exhibited the strongest hydrophilicity (GRAVY = −0.766), while CmPUB11 exhibited the strongest hydrophobicity (GRAVY = 0.193). The subcellular localization prediction results varied considerably, with most proteins predicted to be localized in the nucleus, chloroplasts, and cytoplasm.

3.2. Chromosomal Localization of CmPUBs

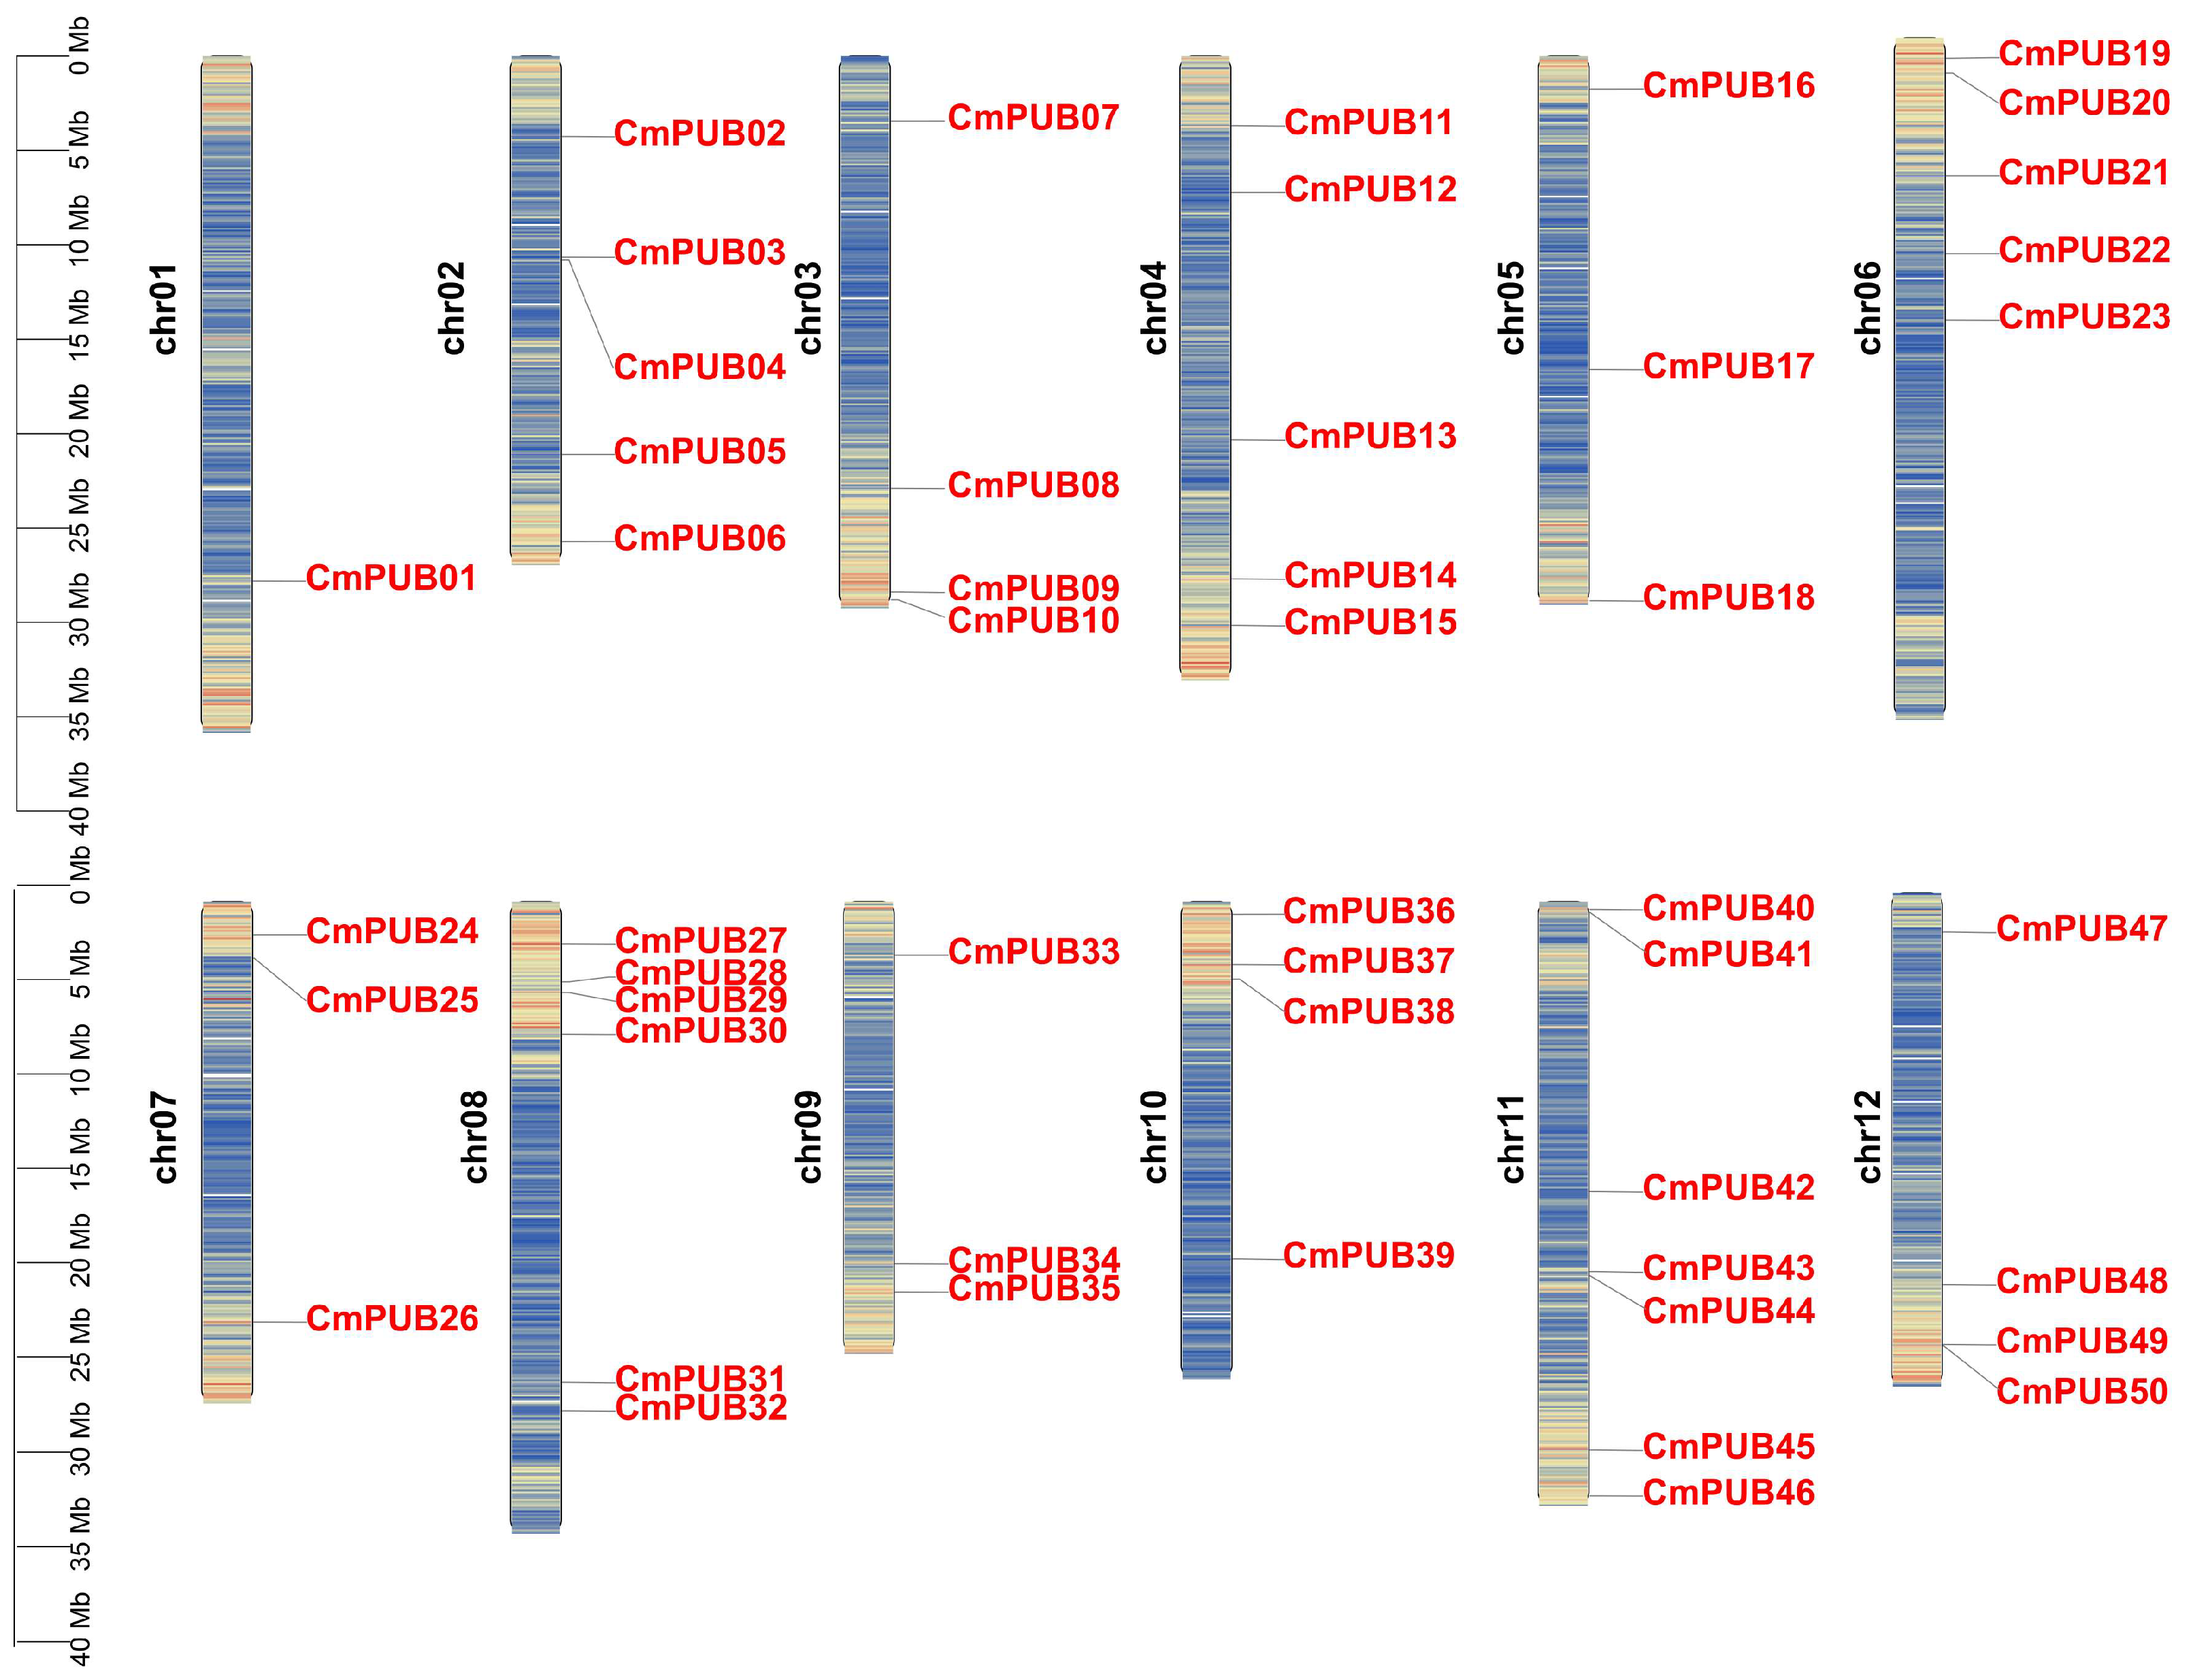
The 50 CmPUBs were unevenly distributed across all 12 melon chromosomes (Figure 1). Among them, chromosomes 8 and 11 contained the highest numbers of CmPUBs, with 6 and 7 genes, respectively; this was followed by chromosomes 2, 4, and 6, each of which contained 5 genes. Chromosomes 3, 10, and 12 each harbored 4 genes, chromosomes 5, 7, and 9 each had 3 genes, and chromosome 1 contained only CmPUB01.

3.3. Motif and Gene Structure Analysis of CmPUBs

To investigate the structural characteristics and evolutionary patterns of CmPUB proteins, we examined their conserved motif composition, domain organization, and gene structural features. CmPUBs exhibited significant differences in the composition of conserved motifs (Figure 2a), but members within the same branch had relatively consistent motif patterns. Overall, Motif 1 and Motif 2 were highly conserved in most members, almost constituting the core motif features of this protein family. Apart from the core motifs, different branches exhibited significant differences in the composition of motifs 3 to 10.
The domains of CmPUBs (Figure 2b) indicated that, in addition to containing the typical U-box domain, CmPUB proteins also comprised various functional domains, such as ARM repeat sequences, WD40 repeat sequences, and other auxiliary regulatory domains. Meanwhile, the presence of WD40 and other domains might further expand their substrate recognition or regulatory functions, thereby forming a multilayered ubiquitination regulatory system.
We also analyzed the exon–intron structures of CmPUBs (Figure 2c). The CmPUBs exhibited extensive structural variation, with a broad range of exon numbers, and most members possessed split gene structures. There was a certain degree of structural conservation among different groups: some branches had relatively simple gene structures with few or no introns, presenting a compact gene architecture; whereas other branches exhibited more complex splicing patterns with an increase in the number of introns and a more dispersed arrangement of exons.

3.4. Phylogenetic Analysis of CmPUBs

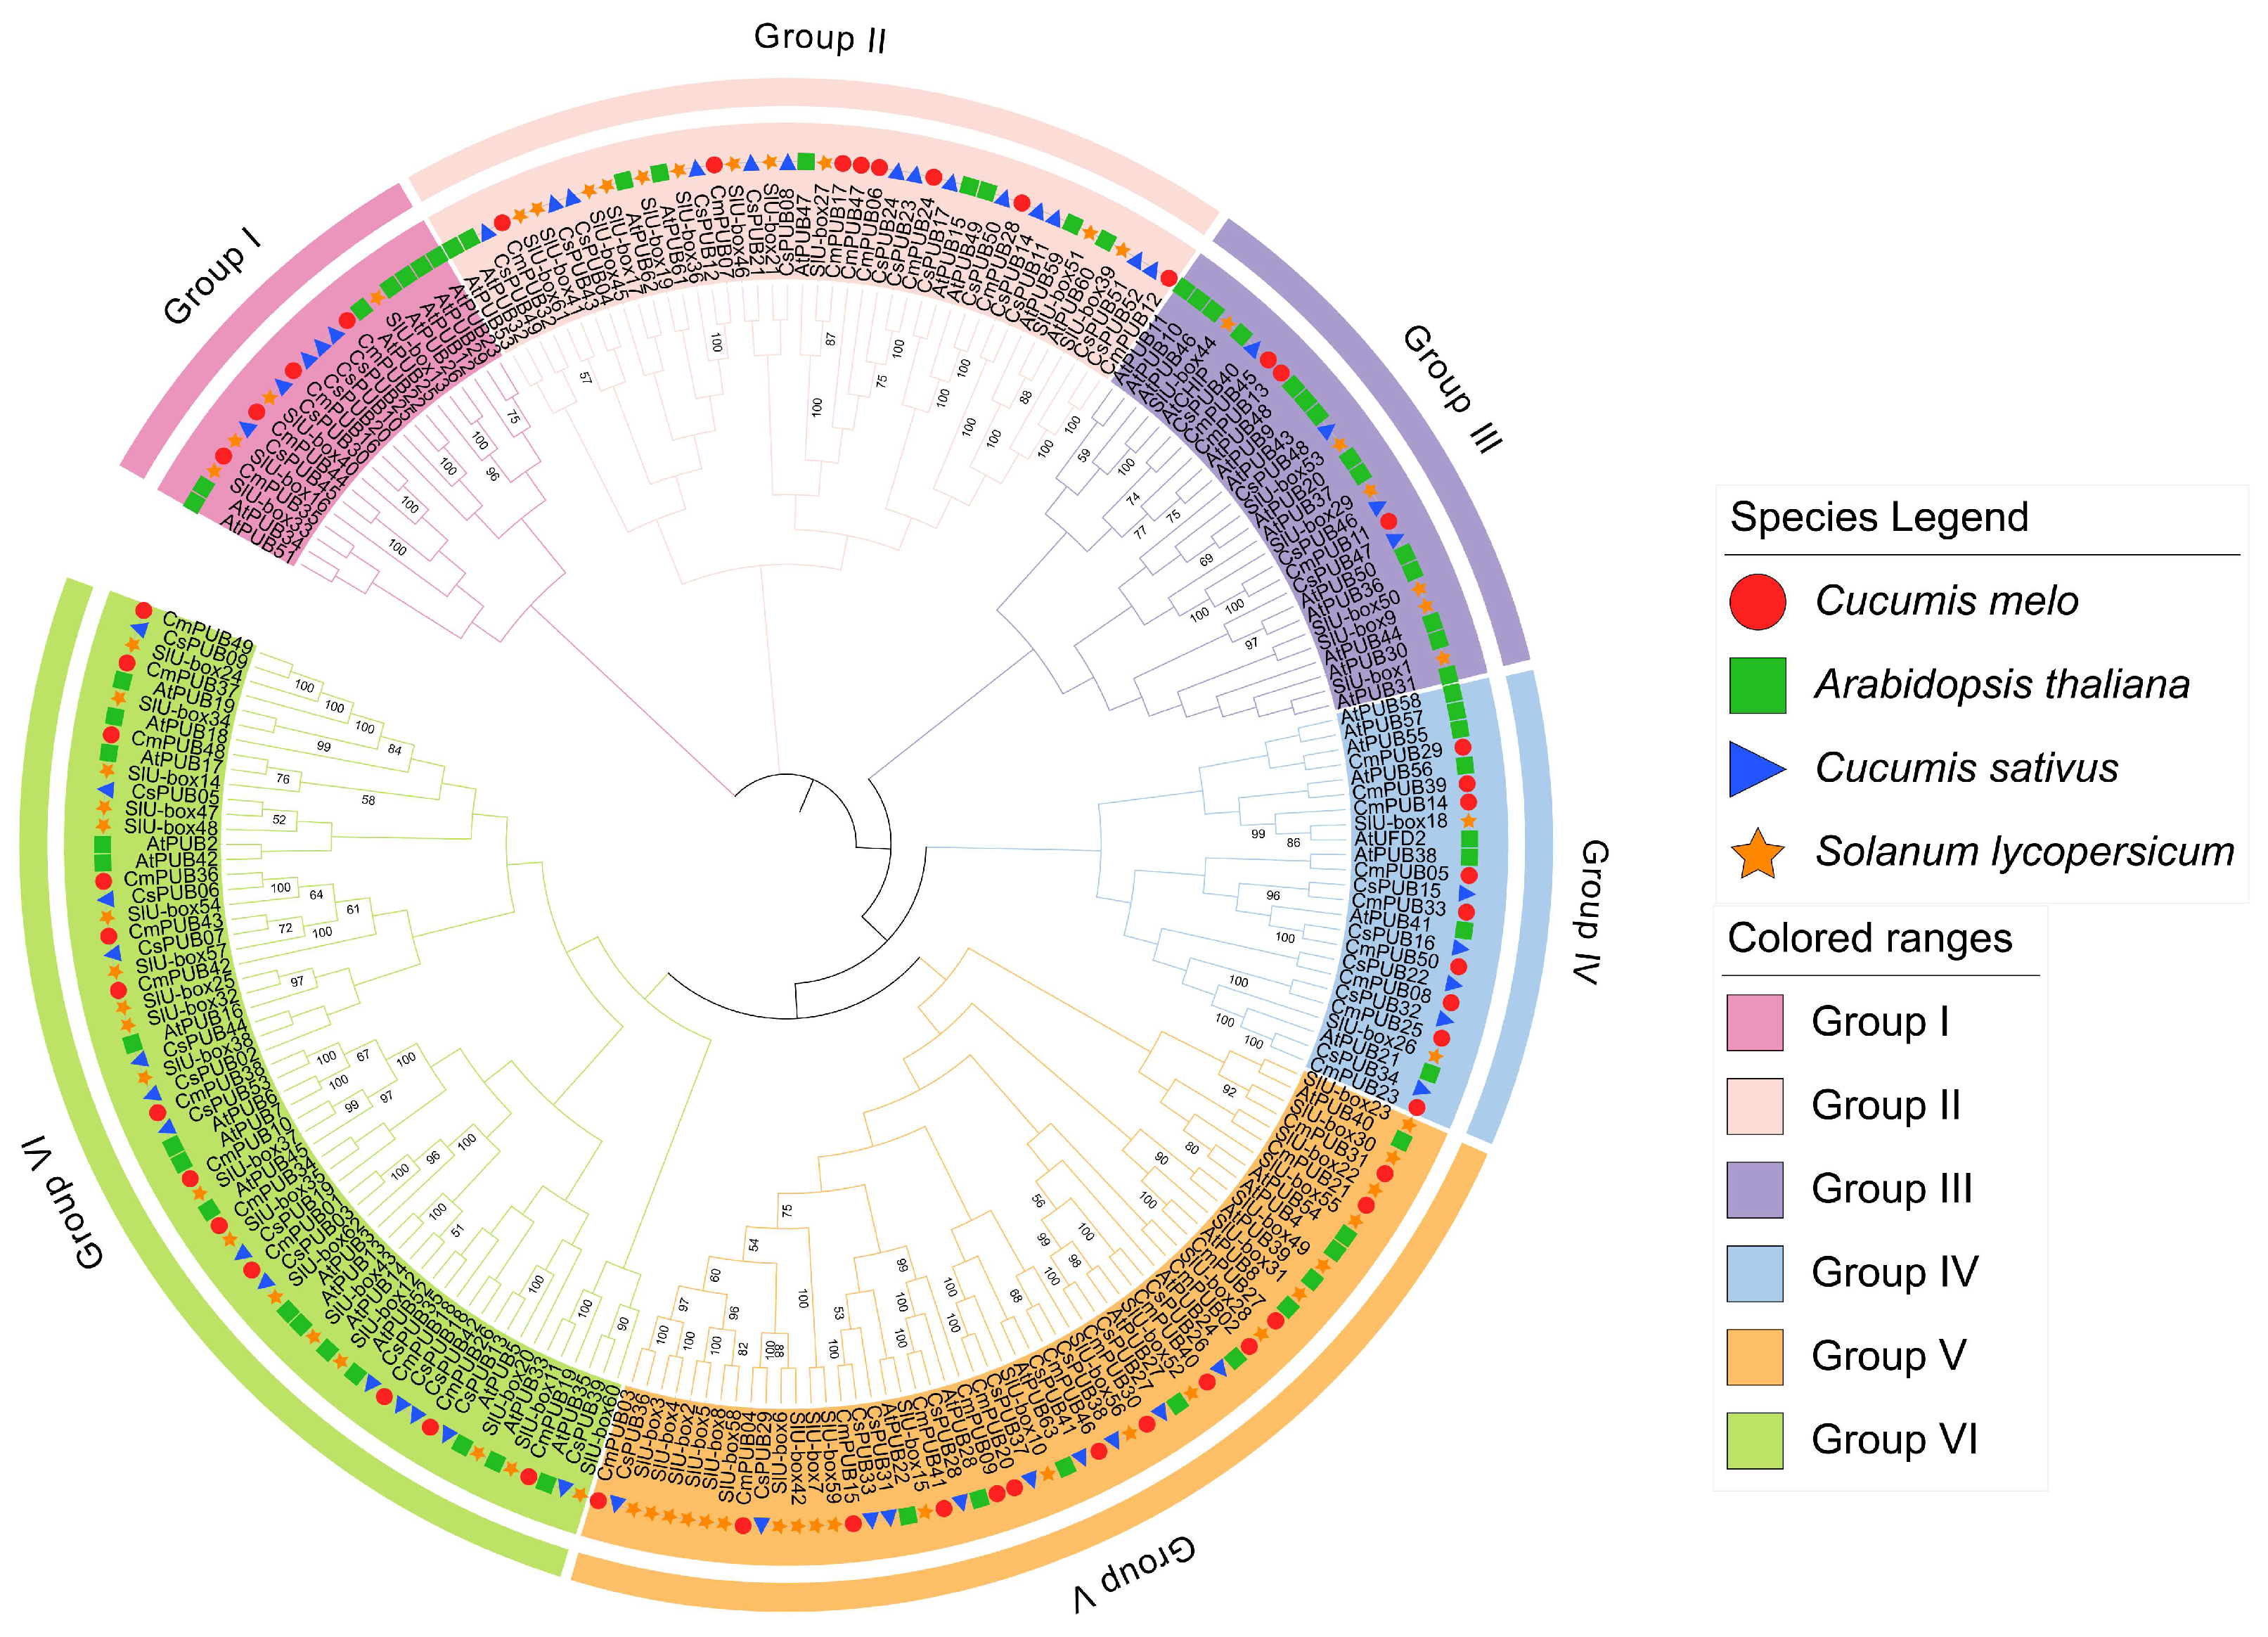
To investigate the relationship between the CmPUB family in melon and the PUB proteins of five species, a phylogenetic relationship was inferred from the alignment of 229 PUB protein sequences obtained from melon, Arabidopsis [28], cucumber [31], and tomato [32] (Figure 3). The results indicated that CmPUBs could be divided into six major subfamilies (Groups I–VI), with uneven distribution among them. Groups V and VI were the two largest subfamilies, each containing 13 CmPUB members, constituting the core groups of this family, whereas Groups I and III contained only 4 and 3 members, respectively.

3.5. Promoter Analysis of CmPUBs

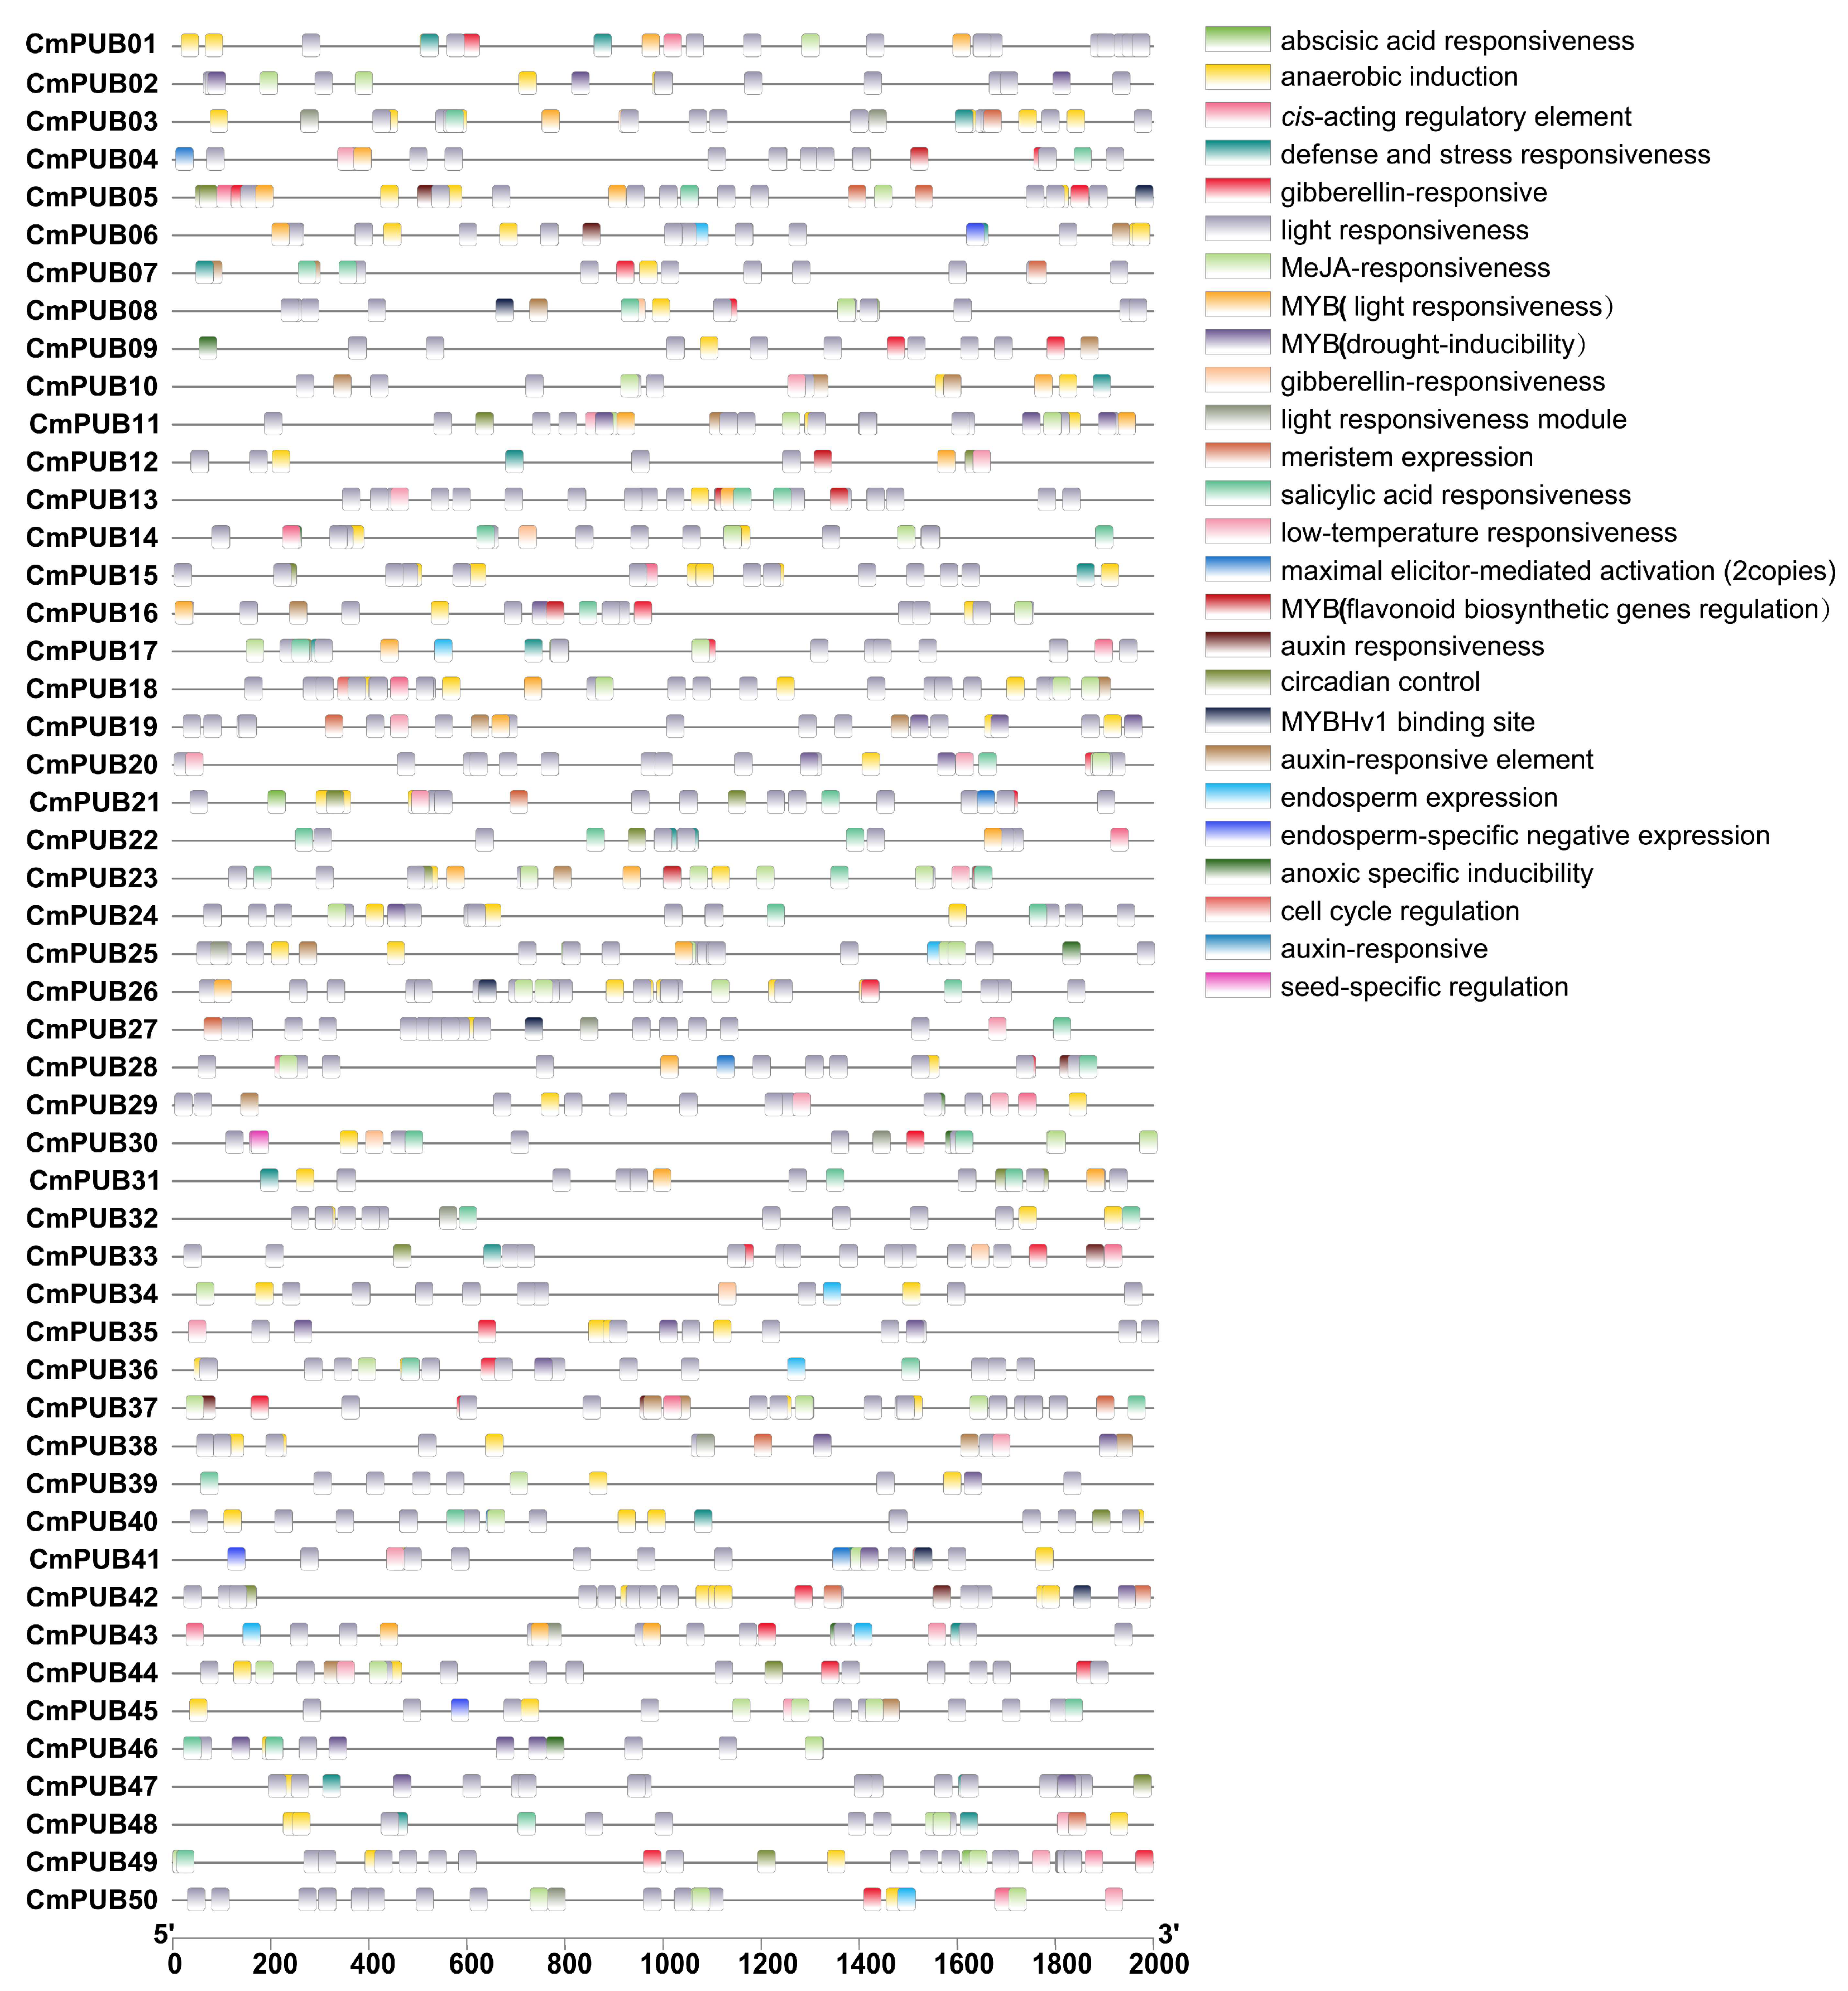
Potential cis-acting regulatory elements located in the promoter regions were characterized (Figure 4), and the results indicated that the promoter regions of CmPUBs were rich in various types of cis-acting elements. These elements could be categorized into the following functional groups: phytohormone-responsive elements, biotic/abiotic stress-responsive elements, light-responsive elements, and elements associated with growth, development, and tissue specificity (Table S5).
A large number of light-responsive elements were present in CmPUBs, indicating that CmPUBs may be commonly involved in the regulation of light signaling. Plant hormone-responsive elements were also widely present, including those responsive to auxin, jasmonic acid (JA), and salicylic acid (SA). In addition, low-temperature-, anaerobic-condition-, drought-, and defense-responsive elements (including MBS, ABRE, ARE, LTR, TC-rich repeats, MYB/MYC binding sites, GC motifs, and WUN motifs) were detected in the promoter regions of multiple CmPUBs. At the same time, cis-acting elements related to circadian rhythm regulation, seed development, and tissue-specific expression were also identified.

3.6. Collinearity Analysis of CmPUBs

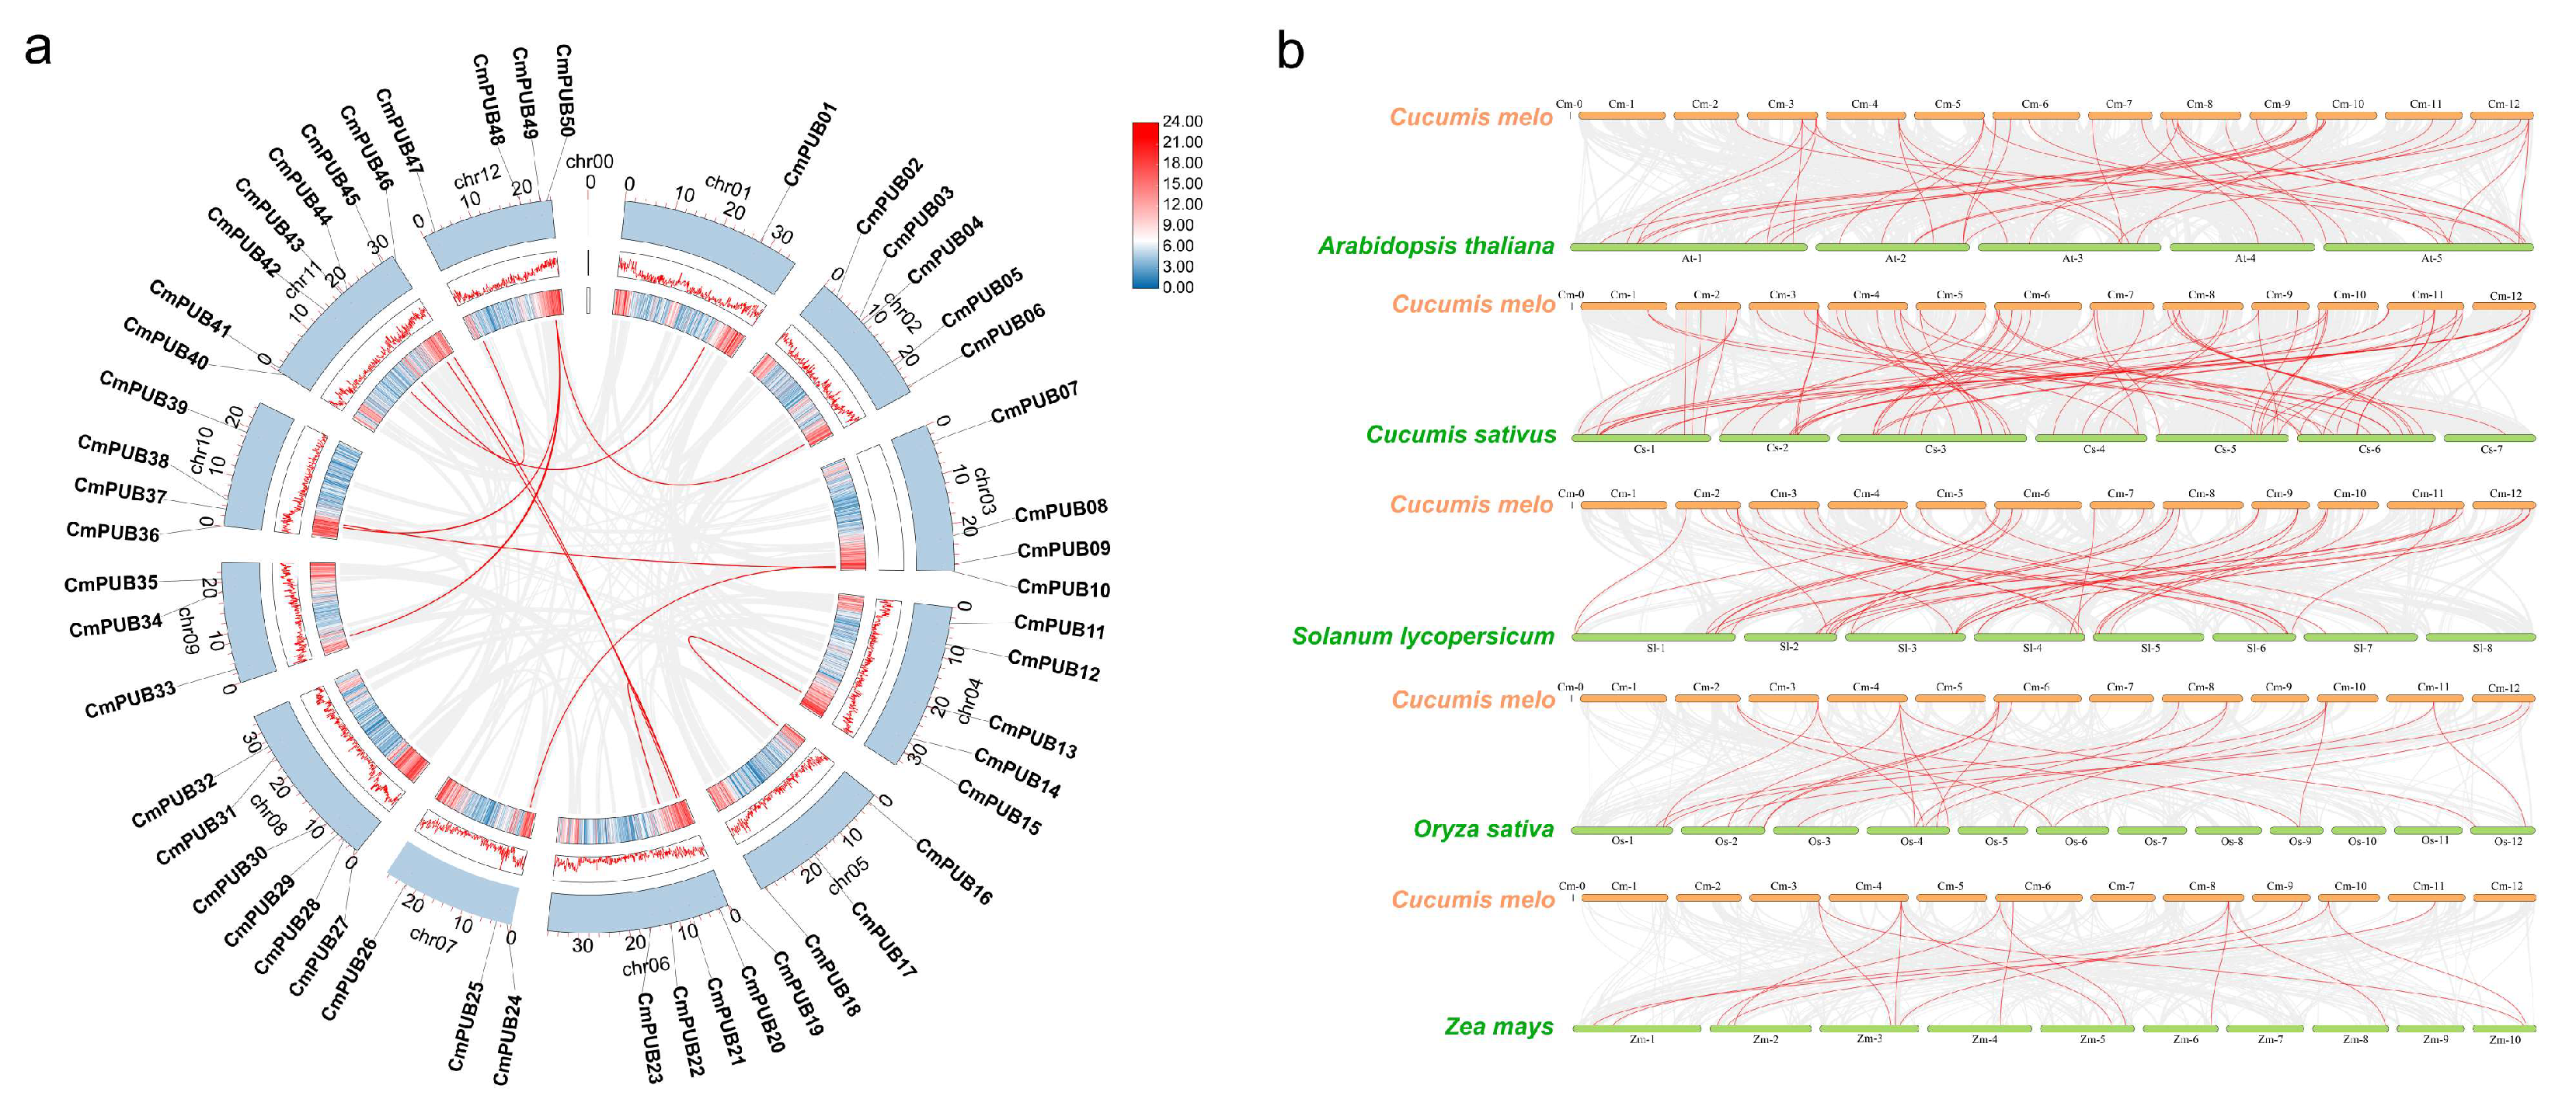
Intraspecific collinearity analysis identified 11 pairs of collinear homologous genes in the CmPUB family (Figure 5a, Table S6), indicating that these genes maintained a high degree of conservation in their nucleotide sequences, and fragment duplication might have been involved in the amplification process of CmPUBs. To elucidate the evolutionary diversification of the CmPUB family, comparative synteny analysis was performed between melon and five species, namely Arabidopsis (A. thaliana), cucumber (C. sativus), tomato (S. lycopersicum), rice (O. sativa), and maize (Z. mays). Interspecific collinearity analysis identified 183 pairs of genes (Table S7), and melon had 39, 67, 40, 22, and 15 pairs of collinear genes with Arabidopsis, cucumber, tomato, rice, and maize, respectively (Figure 5b). These results revealed that as the phylogenetic distance increased, the number of collinear gene pairs showed a gradually decreasing trend, suggesting that the conservation level of PUB gene synteny varied according to the evolutionary distance between different species.

3.7. Protein Structure Analysis of CmPUBs

Among the 50 CmPUB proteins, α-helices were the predominant secondary structural elements. The central regions of these proteins exhibited the typical globular fold characteristic of the U-box family, indicating that their overall structural framework was highly conserved (Figure S2). However, certain variations were observed among different members in terms of helix number, flexible loop length, and spatial assembly, while some short-sequence proteins exhibited relatively streamlined domain architectures, suggesting that the family possessed a structural basis for functional divergence while retaining the core ubiquitin ligase function.

3.8. Expression Patterns of CmPUBs in Response to Salt Stress

To determine an appropriate NaCl concentration for subsequent salt stress treatment, the germination responses of M4-116 and M4-75 were evaluated under different NaCl concentrations (50, 100, 150, and 200 mM). As shown in Table S2, the two cultivars showed distinct germination responses at 150 mM NaCl, with a clear difference in germination rates between M4-116 and M4-75. Based on these results, 150 mM NaCl was selected for subsequent salt stress treatments.
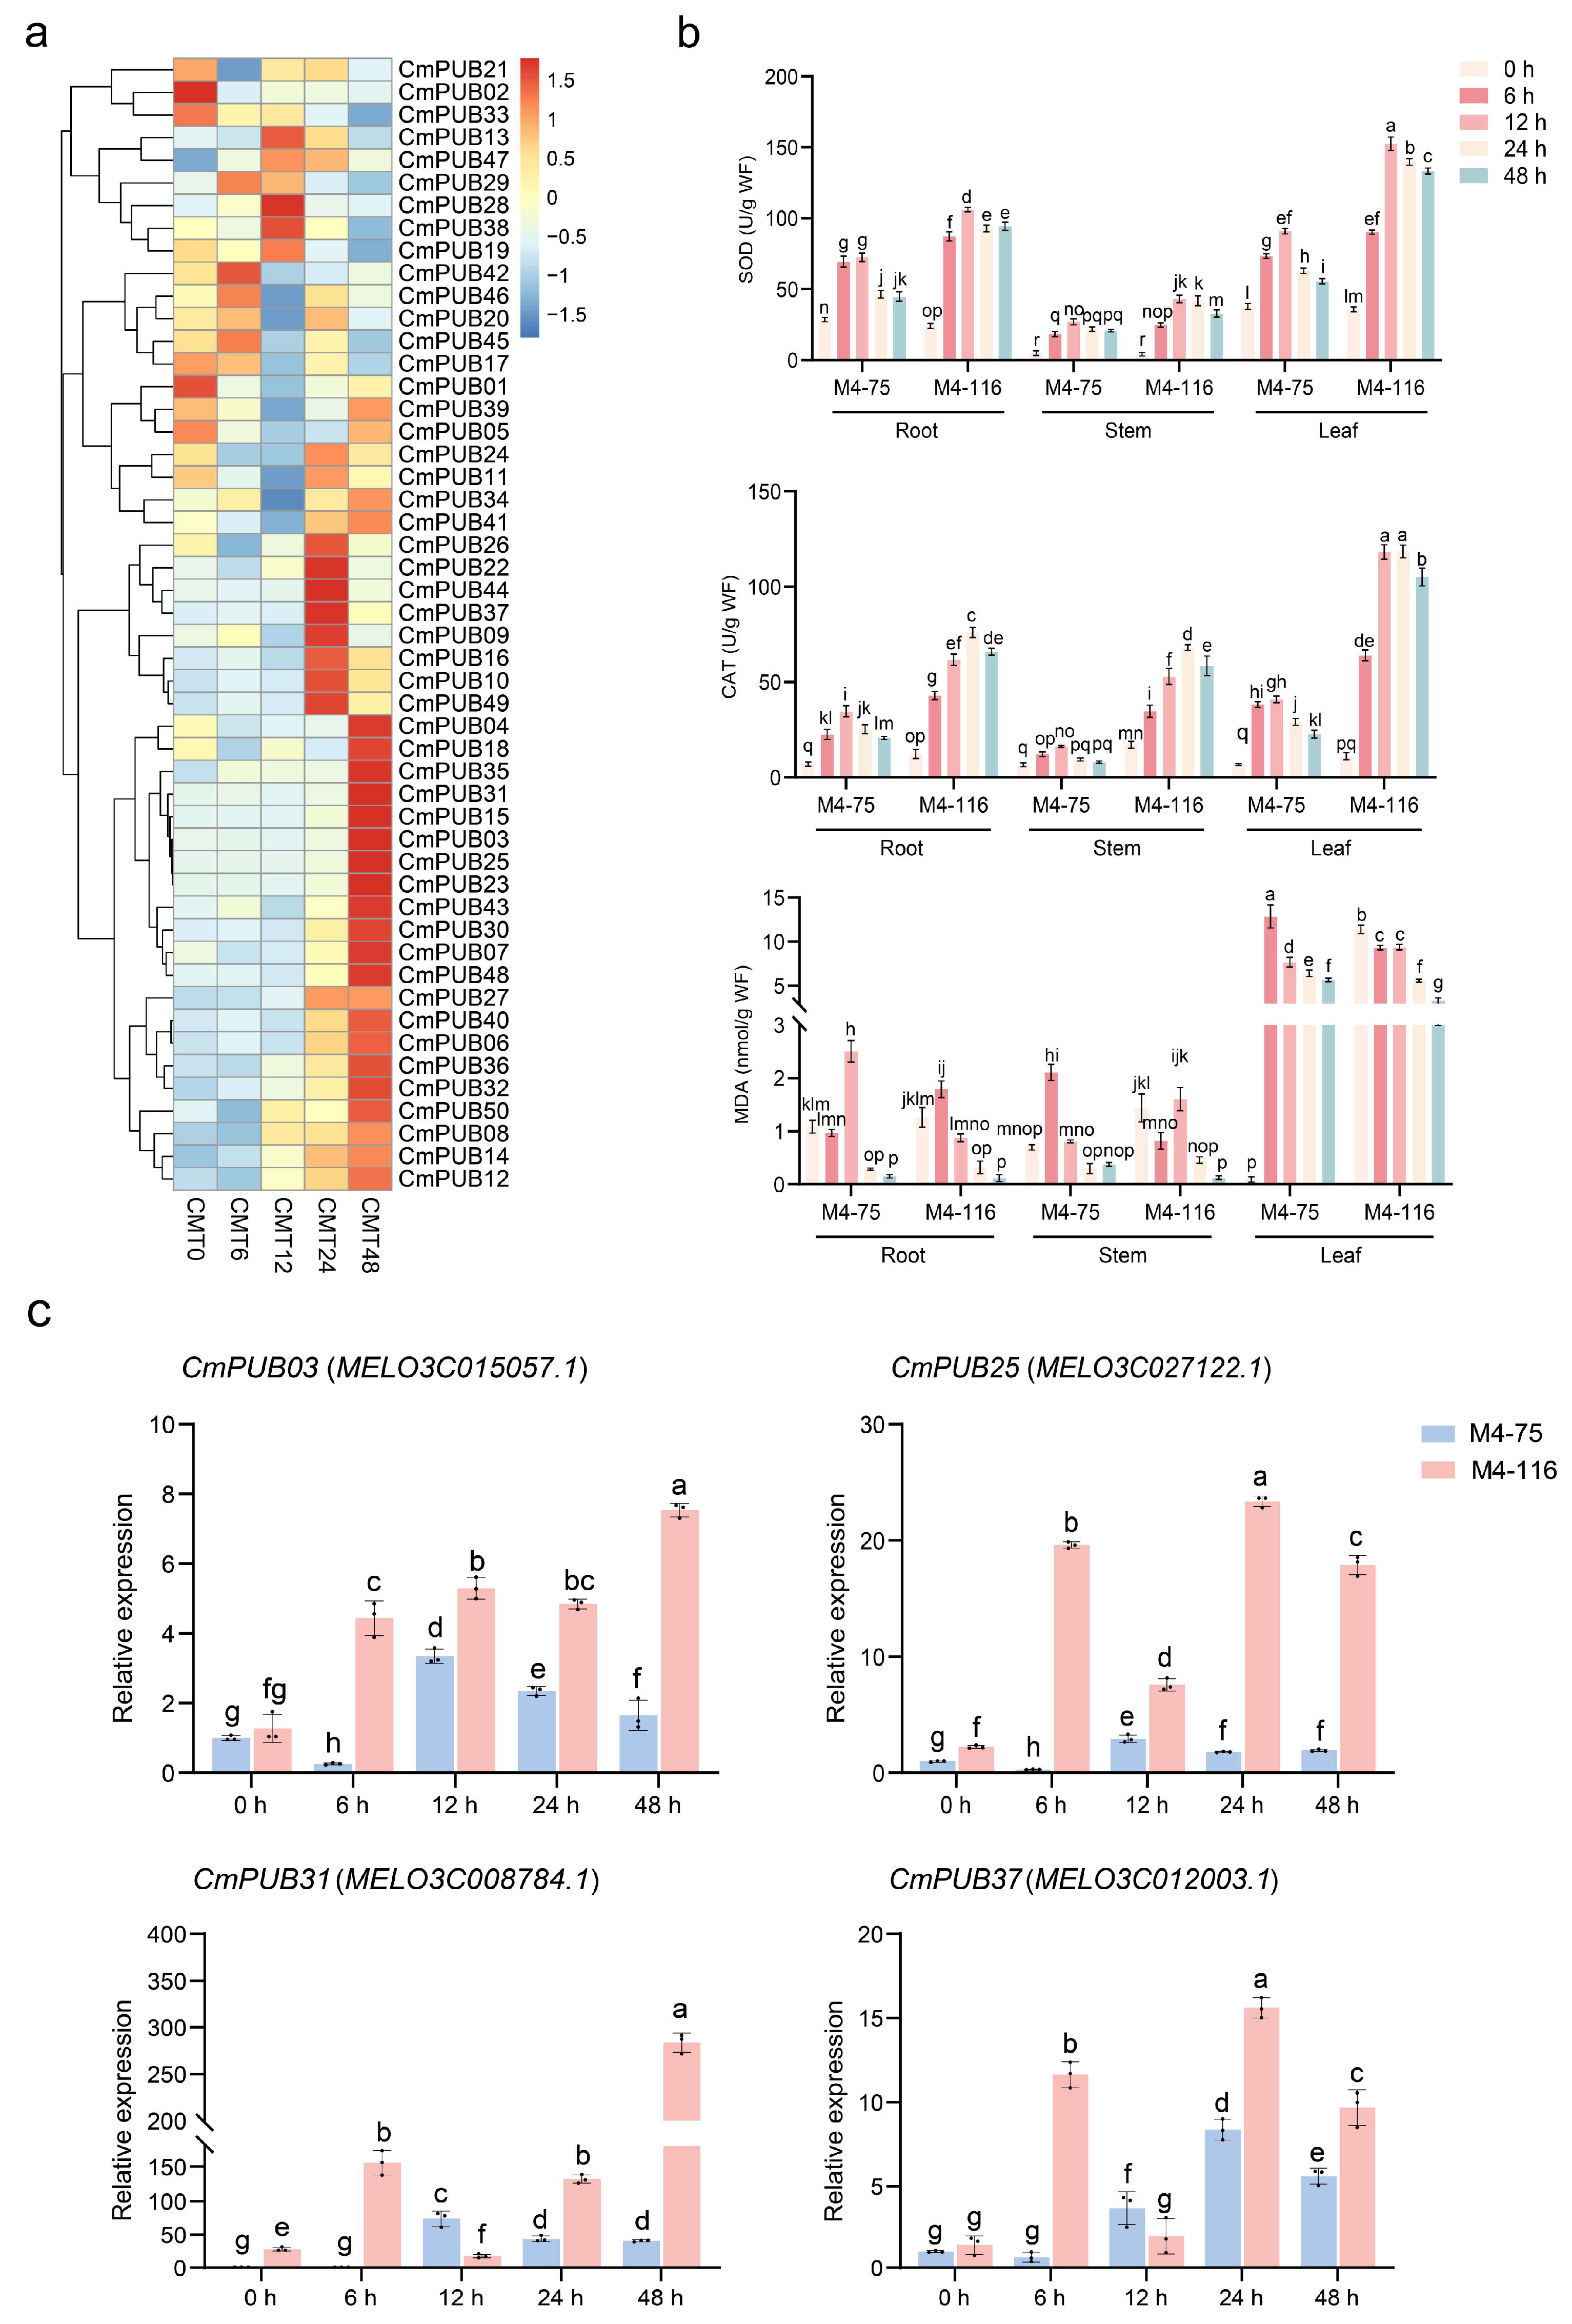
To further elucidate the response of melon to salt stress, we analyzed the expression dynamics of CmPUBs at 0, 6, 12, 24, and 48 h after salt treatment using RNA-Seq data from the melon cultivar ‘Longqing’ under salt stress [43] (Figure 6a). Most CmPUBs exhibited significant differential expression after salt stress treatment, and their expression dynamics at different time points showed notable differences. Some CmPUBs were rapidly activated in the early stages of salt treatment (6 or 12 h), while other genes were continuously and stably upregulated in the subsequent stages (24 or 48 h). This result indicated that CmPUBs might be involved in regulating different temporal stages of the salt stress response.
Salt-tolerant (M4-116) and salt-sensitive (M4-75) melon cultivars were subjected to salt stress, and the SOD and CAT activities and MDA contents in roots, stems, and leaves were measured at different time points. The results showed that leaves were the primary tissues responding to salt-induced oxidative damage in melon, as the changes in all physiological parameters were significantly greater in leaves than in roots and stems (Figure 6b). Compared with M4-75, M4-116 maintained higher SOD and CAT activities and lower MDA accumulation levels during salt stress, indicating that M4-116 could alleviate salt-induced oxidative damage by enhancing its antioxidant defense capacity, thus exhibiting stronger adaptation to salt stress.
Based on the transcriptome screening results, 20 genes highly expressed at the mid-to-late stages of salt stress were selected for qRT-PCR expression validation (Figure 6c and Figure S3). CmPUB03, CmPUB25, CmPUB31, and CmPUB37 were rapidly and strongly induced in the salt-tolerant cultivar M4-116 after 6 h of salt stress, but showed weaker responses in the salt-sensitive cultivar M4-75 (Figure 6c); meanwhile, some genes displayed varying expression differences between the two cultivars.

4. Discussion

Although the PUB gene family has been identified genome-wide in various plants, the composition and expression patterns of PUB members still differ across species, making genome-level family identification insufficient to reflect their potential roles under specific stress conditions. Based on the DHL92 (version 4.0) melon reference genome, this study systematically identified the CmPUB gene family, obtaining 50 CmPUB genes containing complete U-box domains, and further analyzed their salt stress response characteristics. The family size of CmPUBs is comparable to that of the closely related species cucumber (53 CsPUBs) [31], but slightly smaller than those of tomato (62 SlPUBs) [32] and Arabidopsis (64 AtPUBs) [28]. The differences in family size among species likely reflect differential rates of gene retention and loss following lineage-specific whole-genome duplication (WGD) events during plant evolution [49]. Intraspecies collinearity analysis identified 11 collinear gene pairs of CmPUBs located on different chromosomes, indicating that segmental duplication is the primary means of expansion for the PUB family in melon [50,51]. This expansion pattern is consistent with findings in tomato, where segmental duplication generated 10 collinear gene pairs and contributed to family diversification. In contrast, only seven CsPUBs collinear gene pairs were identified in cucumber. This difference suggests that following the lineage-specific ancient polyploidization event in the Cucurbitaceae, the melon genome has retained more duplicated copies of PUB family genes over the course of long-term evolution. Previous studies have confirmed that the common ancestor of Cucurbitaceae plants successively experienced two ancient polyploidization events [52,53,54]. The collinear homologous genes retained in the melon PUB family represent the evolutionary imprints left by these ancient duplication events on the genome.
In this study, we found that the exon–intron structures of CmPUBs varied considerably, ranging from intronless genes to those with multiple introns, which is closely associated with functional divergence [55]. The occurrence of intronless PUB genes has also been reported in grapevine [56], tomato [32] and cucumber [31]. It is generally recognized that intronless genes can facilitate rapid transcriptional responses by avoiding the requirement for pre-mRNA splicing, and they are often preferentially associated with stress-responsive expression [57], whereas multi-intron genes can generate transcript diversity through alternative splicing, and their introns may act as a buffer to reduce the probability of deleterious mutations in coding regions [58]. There are two distinct structural architectures within the CmPUB family, indicating that a sophisticated regulatory system has evolved within this family, balancing rapid stress responses with long-term evolutionary resilience. Analysis of conserved motifs uncovered 10 separate motifs in CmPUB proteins; the motif matching the U-box domain appears in every family member, while the remaining motifs exhibited subfamily-specific distribution. This motif arrangement is highly consistent with the findings in tomato [32] and sorghum [59], providing further evidence for the structural conservation of the PUB family in angiosperms. Phylogenetic analysis results indicate that three PUB genes in melon—CmPUB37, CmPUB48, and CmPUB49—form a close evolutionary branch with Arabidopsis AtPUB18 and AtPUB19, and previous studies have confirmed that the latter two are involved in the salt stress response process [25]. Collinearity analysis also confirmed that the homologous genes of melon and Arabidopsis PUB are highly conserved, indicating that their core functions have been largely preserved throughout evolution. Combining phylogenetic relationships with gene expression data to identify salt-tolerant candidate genes is a common approach in cucurbit research. For example, researchers have successfully screened relevant members of the cucumber LRX family by using evolutionary conservation and stress-induced expression patterns [60].
To further investigate the involvement of CmPUBs in salt stress responses, transcriptome, qRT-PCR, and physiological analyses were integrated. The RNA-Seq dataset from the melon cultivar ‘Longqing’ [43] revealed distinct temporal expression patterns among multiple CmPUB genes following salt treatment, with some members responding predominantly at early stages and others showing greater changes at later stages. Based on the transcriptome screening results, 20 CmPUB genes were selected for qRT-PCR analysis in the salt-tolerant cultivar M4-116 and salt-sensitive cultivar M4-75. Among these genes, CmPUB03, CmPUB25, CmPUB31, and CmPUB37 showed stronger induction in M4-116, particularly at 6 h after salt treatment. The enhanced expression of these genes in the salt-tolerant cultivar, together with their salt-responsive expression patterns, suggests their potential association with differential responses to salt stress. Notably, the RNA-Seq data were obtained from ‘Longqing’, whereas the qRT-PCR and physiological experiments were conducted using M4-116 and M4-75, and therefore these datasets provide complementary evidence across different genetic backgrounds. Salt stress commonly induces excessive ROS accumulation and oxidative damage, and antioxidant enzymes such as SOD and CAT play important roles in maintaining cellular redox balance. In the present study, M4-116 maintained higher SOD and CAT activities and lower MDA accumulation than M4-75 under salt stress, particularly in leaves, indicating stronger antioxidant capacity and reduced membrane lipid peroxidation in the salt-tolerant cultivar. Similar associations between enhanced antioxidant defense and salt tolerance have been reported in watermelon, pumpkin, tomato, apple, and bok choy [61,62,63,64,65,66,67,68]. For example, the ClWRKY6–ClLEA55 module in watermelon was associated with enhanced ROS-scavenging capacity under salt stress [61], whereas CmoDREB2A was reported to participate in salt adaptation through the regulation of hydrogen peroxide signaling, abscisic acid-related responses, and K+/Na+ homeostasis [62]. These findings provide a broader physiological context for the antioxidant responses observed between M4-116 and M4-75. The stronger expression of CmPUB03, CmPUB25, CmPUB31, and CmPUB37 in M4-116 occurred in parallel with these physiological differences, supporting their association with salt-responsive processes in melon.
The transcriptome and cultivar-based experiments were performed using different melon genetic backgrounds, and the physiological measurements were primarily focused on SOD, CAT, and MDA. Other important components of salt tolerance, including ROS accumulation, Na+/K+ homeostasis, ion transport, osmotic adjustment, and hormone signaling, were not directly examined in relation to individual CmPUB genes. Thus, the observed transcriptional and physiological changes provide complementary evidence for candidate-gene prioritization but do not establish direct regulatory relationships. Future functional studies using VIGS [69], CRISPR/Cas9-mediated gene editing [70], and overexpression, together with analyses of ROS homeostasis, ion balance, protein interactions, and ubiquitination substrates, will help clarify the molecular functions of these CmPUB genes. Overall, CmPUB03, CmPUB25, CmPUB31, and CmPUB37 represent promising candidate genes associated with salt stress responses in melon and provide a basis for further investigation of PUB-mediated salt stress regulation.

5. Conclusions

This study conducted a whole-genome screening and identified 50 CmPUBs, all of which contain a complete U-box domain. These genes were unevenly distributed across the 12 chromosomes and exhibited considerable diversity in gene structures, conserved motifs, and domain compositions. Phylogenetic and collinearity analyses revealed the evolutionary relationships and duplication patterns of the CmPUB family, while promoter analysis indicated the presence of diverse hormone- and stress-responsive cis-acting elements. Transcriptome and qRT-PCR analyses further showed that multiple CmPUB genes responded to salt stress, and CmPUB03, CmPUB25, CmPUB31, and CmPUB37 exhibited stronger induction in the salt-tolerant cultivar M4-116 than in the salt-sensitive cultivar M4-75. These expression patterns, together with the differences in antioxidant enzyme activities and MDA accumulation between the two cultivars, suggest that these genes are promising candidates associated with salt stress responses in melon. Overall, this study provides a comprehensive genomic characterization of the CmPUB family and identifies candidate CmPUB genes for further functional investigation and molecular breeding for salt tolerance in melon.

Supplementary Materials

The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/horticulturae12101215/s1; Table S1: PUB genes identified in different plant species; Table S2: Seed germination rate under different NaCl concentrations; Table S3: List of qRT-PCR primers of CmPUBs; Table S4: Information on PUB family genes in melon; Table S5: Statistical analysis of the number of cis-acting elements of CmPUBs; Table S6: Intraspecies collinearity analysis of the CmPUB gene family; Table S7: Interspecific collinearity analysis between melon and five reference species; Figure S1. PRISMA-style flowchart illustrating the identification and screening procedure of the CmPUB gene family in melon; Figure S2: Prediction of three-dimensional structures of CmPUBs; Figure S3: qRT-PCR validation of 16 CmPUBs from the RNA-seq data (PRJNA987131).

Author Contributions

Conceptualization, X.F.; methodology, X.F.; software, Y.L.; validation, Y.L. and Z.L.; formal analysis, F.L. (Fanzhuo Lin); investigation, Y.L., Z.H., and X.F.; resources, F.L.(Feishi Luan); data curation, Y.L., F.L. (Fanzhuo Lin), and Z.H.; writing—original draft preparation, Y.L.; writing—review and editing, X.F.; visualization, Z.L.; supervision, S.L.; project administration, X.F.; funding acquisition, X.W., S.L., and X.F. All authors have read and agreed to the published version of the manuscript.

Funding

This research was funded by the National Natural Science Foundation of China (grant number: U25A20690), the National Natural Science Foundation of China (grant number: 32472747), the Program for Young Talents of Basic Research in Universities of Heilongjiang Province (grant number: YQJH2024012), the Talent Introduction Project of Northeast Agricultural University (grant number: 24YJQA02), the Postdoctoral Program of Heilongjiang Province (grant number: LBH-Z25066) and the China Agriculture Research System of MOF and MARA (grant number: CARS-25).

Data Availability Statement

The original contributions presented in this study are included in the Supplementary Material. Further inquiries can be directed to the corresponding authors.

Acknowledgments

We appreciate all the people who have collaborated on this project.

Conflicts of Interest

The authors declare no conflicts of interest.

References

  1. Chikh-Rouhou, H.; Abdedayem, W.; Solmaz, I.; Sari, N.; Garcés-Claver, A. Melon (Cucumis melo L.): Genomics and Breeding. In Smart Plant Breeding for Vegetable Crops in Post-Genomics Era; Springer: Berlin/Heidelberg, Germany, 2023; pp. 25–52. [Google Scholar]
  2. Wang, P.; Zhu, L.; Li, Z.; Cheng, M.; Chen, X.; Wang, A.; Wang, C.; Zhang, X. Genome-wide identification of the U-box E3 ubiquitin ligase gene family in cabbage (Brassica oleracea var. capitata) and its expression analysis in response to cold stress and pathogen infection. Plants 2023, 12, 1437. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  3. Su, Y.; Ngea, G.L.N.; Wang, K.; Lu, Y.; Godana, E.A.; Ackah, M.; Yang, Q.; Zhang, H. Deciphering the mechanism of E3 ubiquitin ligases in plant responses to abiotic and biotic stresses and perspectives on PROTACs for crop resistance. Plant Biotechnol. J. 2024, 22, 2811–2843. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  4. Hua, Z. The Ubiquitin–26S Proteasome System—A Versatile Player Worthy of Close Attention in Plants. Int. J. Mol. Sci. 2023, 24, 8185. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  5. Langin, G.; González-Fuente, M.; Üstün, S. The Plant Ubiquitin–Proteasome System as a Target for Microbial Manipulation. Annu. Rev. Phytopathol. 2023, 61, 351–375. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  6. Stone, S.L. Ubiquitin Ligases at the Nexus of Plant Responses to Biotic and Abiotic Stresses. Essays Biochem. 2022, 66, 123–133. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  7. Diehl, C.J.; Ciulli, A. Discovery of small molecule ligands for the von Hippel-Lindau (VHL) E3 ligase and their use as inhibitors and PROTAC degraders. Chem. Soc. Rev. 2022, 51, 8216–8257. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  8. Karki, R.; Gadiya, Y.; Shetty, S.; Gribbon, P.; Zaliani, A. Pharmacophore-based ML model to filter candidate E3 ligands and predict E3 ligase binding probabilities. Inform. Med. Unlocked 2024, 44, 101424. [Google Scholar] [CrossRef] [Scilit]
  9. Sierra-Cacho, D.; Méndez-Gómez, M.; Aguilar-Hernández, V.; Guzmán, P. Functional Diversity of A-Type RING Ligases (ATL) Genes: Insights into the Crucial Roles of E3 Ubiquitin Ligases in Plant Biology. J. Plant Growth Regul. 2025, 44, 1827–1845. [Google Scholar] [CrossRef] [Scilit]
  10. Park, C.-R.; Min, J.-H.; Gong, Y.; Sang, H.; Lee, K.-H.; Kim, C.S. Arabidopsis thaliana ubiquitin-associated protein 2 (AtUAP2) functions as an E4 ubiquitin factor and negatively modulates dehydration stress response. Plant Mol. Biol. 2024, 114, 13. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  11. Metzger, M.B.; Pruneda, J.N.; Klevit, R.E.; Weissman, A.M. RING-type E3 ligases: Master manipulators of E2 ubiquitin-conjugating enzymes and ubiquitination. Biochim. Biophys. Acta 2014, 1843, 47–60. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  12. Trenner, J.; Monaghan, J.; Saeed, B.; Quint, M.; Shabek, N.; Trujillo, M. Evolution and Functions of Plant U-Box Proteins: From Protein Quality Control to Signaling. Annu. Rev. Plant Biol. 2022, 73, 93–121. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  13. Trujillo, M. News from the PUB: Plant U-box type E3 ubiquitin ligases. J. Exp. Bot. 2018, 69, 371–384. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  14. Suranjika, S.; Barla, P.; Sharma, N.; Dey, N. A review on ubiquitin ligases: Orchestrators of plant resilience in adversity. Plant Sci. 2024, 347, 112180. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  15. Mao, X.; Yu, C.; Li, L.; Wang, M.; Yang, L.; Zhang, Y.; Zhang, Y.; Wang, J.; Li, C.; Reynolds, M.P.; et al. How Many Faces Does the Plant U-Box E3 Ligase Have? Int. J. Mol. Sci. 2022, 23, 2285. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  16. Feng, H.; Tan, J.; Deng, Z. Decoding plant adaptation: Deubiquitinating enzymes UBP12 and UBP13 in hormone signaling, light response, and developmental processes. J. Exp. Bot. 2024, 75, 721–732. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  17. Santner, A.; Estelle, M. The ubiquitin-proteasome system regulates plant hormone signaling. Plant J. 2010, 61, 1029–1040. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  18. Hasegawa, Y.; Luo, Y.; Sato, T. Recent Advances in Ubiquitin Signals Regulating Plant Membrane Trafficking. Plant Cell Physiol. 2024, 65, 1907–1924. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  19. Hamada, N.; Hand, K.A.; Shabek, N. Ubiquitin ligases in plant immunity: Structural mechanisms and signaling. Plant J. 2026, 126, e70846. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  20. Xu, J.; Liu, H.; Zhou, C.; Wang, J.; Wang, J.; Han, Y.; Zheng, N.; Zhang, M.; Li, X. The ubiquitin-proteasome system in the plant response to abiotic stress: Potential role in crop resilience improvement. Plant Sci. 2024, 342, 112035. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  21. Wang, S.; Lv, X.; Zhang, J.; Chen, D.; Chen, S.; Fan, G.; Ma, C.; Wang, Y. Roles of E3 ubiquitin ligases in plant responses to abiotic stresses. Int. J. Mol. Sci. 2022, 23, 2308. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  22. Chen, X.; Wang, T.; Rehman, A.U.; Wang, Y.; Qi, J.; Li, Z.; Song, C.; Wang, B.; Yang, S.; Gong, Z. Arabidopsis U-box E3 ubiquitin ligase PUB11 negatively regulates drought tolerance by degrading the receptor-like protein kinases LRR1 and KIN7. J. Integr. Plant Biol. 2021, 63, 494–509. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  23. Zhao, J.; Zhao, L.; Zhang, M.; Zafar, S.A.; Fang, J.; Li, M.; Zhang, W.; Li, X. Arabidopsis E3 ubiquitin ligases PUB22 and PUB23 negatively regulate drought tolerance by targeting ABA receptor PYL9 for degradation. Int. J. Mol. Sci. 2017, 18, 1841. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  24. Qin, Q.; Wang, Y.; Huang, L.; Du, F.; Zhao, X.; Li, Z.; Wang, W.; Fu, B. A U-box E3 ubiquitin ligase OsPUB67 is positively involved in drought tolerance in rice. Plant Mol. Biol. 2020, 102, 89–107. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  25. Bergler, J.; Hoth, S. Plant U-box armadillo repeat proteins AtPUB18 and AtPUB19 are involved in salt inhibition of germination in Arabidopsis. Plant Biol. 2011, 13, 725–730. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  26. Li, Q.; Li, B.; Wang, J.; Chang, X.; Mao, X.; Jing, R. TaPUB15, a U-box E3 ubiquitin ligase gene from wheat, enhances salt tolerance in rice. Food Energy Secur. 2021, 10, e250. [Google Scholar] [CrossRef] [Scilit]
  27. Wang, X.; Ding, Y.; Li, Z.; Shi, Y.; Wang, J.; Hua, J.; Gong, Z.; Zhou, J.-M.; Yang, S. PUB25 and PUB26 promote plant freezing tolerance by degrading the cold signaling negative regulator MYB15. Dev. Cell 2019, 51, 222–235.e5. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  28. Wiborg, J.; O’Shea, C.; Skriver, K. Biochemical function of typical and variant Arabidopsis thaliana U-box E3 ubiquitin-protein ligases. Biochem. J. 2008, 413, 447–457. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  29. Zeng, L.R.; Park, C.H.; Venu, R.C.; Gough, J.; Wang, G.L. Classification, expression pattern, and E3 ligase activity assay of rice U-box-containing proteins. Mol. Plant. 2008, 1, 800–815. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  30. Chen, R.; Gu, G.; Zhang, B.; Du, C.; Lin, X.; Cai, W.; Zheng, Y.; Li, T.; Wang, R.; Xie, X. Genome-wide identification and expression analysis of the U-box E3 ubiquitin ligase gene family related to bacterial wilt resistance in tobacco (Nicotiana tabacum L.) and eggplant (Solanum melongena L.). Front. Plant Sci. 2024, 15, 1425651. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  31. Chen, Q.; Zhao, T.; Song, H.; Sha, S.; Ma, J.; Zhang, R.; Kong, W.; Yang, S.; Liu, J.; Wang, Y. Genome-wide identification, characterization, and expression analysis of the U-box gene family in cucumber (Cucumis sativus). Plants 2025, 14, 1801. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  32. Sharma, B.; Taganna, J. Genome-wide analysis of the U-box E3 ubiquitin ligase enzyme gene family in tomato. Sci. Rep. 2020, 10, 9581. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  33. Ryu, M.Y.; Cho, S.K.; Hong, Y.; Kim, J.; Kim, J.H.; Kim, G.M.; Chen, Y.J.; Knoch, E.; Møller, B.L.; Kim, W.T.; et al. Classification of barley U-box E3 ligases and their expression patterns in response to drought and pathogen stresses. BMC Genom. 2019, 20, 326. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  34. Wang, N.; Liu, Y.; Cong, Y.; Wang, T.; Zhong, X.; Yang, S.; Li, Y.; Gai, J. Genome-wide identification of soybean U-box E3 ubiquitin ligases and roles of GmPUB8 in negative regulation of drought stress response in Arabidopsis. Plant Cell Physiol. 2016, 57, 1189–1209. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  35. Zhou, X.; Li, Y.; Wang, J.; Zhao, Y.; Wang, H.; Han, Y.; Lin, X. Genome-wide identification of U-box gene family and expression analysis in response to saline-alkali stress in foxtail millet (Setaria italica L. Beauv). Front. Genet. 2024, 15, 1356807. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  36. Castanera, R.; Ruggieri, V.; Pujol, M.; Garcia-Mas, J.; Casacuberta, J.M. An improved melon reference genome with single-molecule sequencing uncovers a recent burst of transposable elements with potential impact on genes. Front. Plant Sci. 2020, 10, 1815. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  37. Paysan-Lafosse, T.; Andreeva, A.; Blum, M.; Chuguransky, S.R.; Grego, T.; Lazaro Pinto, B.; Salazar, G.A.; Bileschi, M.L.; Llinares-López, F.; Meng-Papaxanthos, L.; et al. The Pfam protein families database: Embracing AI/ML. Nucleic Acids Res. 2025, 53, D523–D534. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  38. Chen, C.; Wu, Y.; Li, J.; Wang, X.; Zeng, Z.; Xu, J.; Liu, Y.; Feng, J.; Chen, H.; He, Y.; et al. TBtools-II: A “one for all, all for one” bioinformatics platform for biological big-data mining. Mol. Plant 2023, 16, 1733–1742. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  39. Bailey, T.L.; Johnson, J.; Grant, C.E.; Noble, W.S. The MEME Suite. Nucleic Acids Res. 2015, 43, W39–W49. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  40. Tamura, K.; Stecher, G.; Kumar, S. MEGA11: Molecular Evolutionary Genetics Analysis version 11. Mol. Biol. Evol. 2021, 38, 3022–3027. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  41. Letunic, I.; Bork, P. Interactive Tree of Life (iTOL) v6: Recent updates to the phylogenetic tree display and annotation tool. Nucleic Acids Res. 2024, 52, W78–W82. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  42. Lescot, M.; Déhais, P.; Thijs, G.; Marchal, K.; Moreau, Y.; Van de Peer, Y.; Rouzé, P.; Rombauts, S. PlantCARE, a database of plant cis-acting regulatory elements and a portal to tools for in silico analysis of promoter sequences. Nucleic Acids Res. 2002, 30, 325–327. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  43. Liu, T.; Amanullah, S.; Xu, H.; Gao, P.; Du, Z.; Hu, X.; Han, M.; Che, Y.; Zhang, L.; Qi, G.; et al. RNA-Seq identified putative genes conferring photosynthesis and root development of melon under salt stress. Genes 2023, 14, 1728. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  44. Chen, S.; Zhou, Y.; Chen, Y.; Gu, J. fastp: An ultra-fast all-in-one FASTQ preprocessor. Bioinformatics 2018, 34, i884–i890. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  45. Kim, D.; Paggi, J.M.; Park, C.; Bennett, C.; Salzberg, S.L. Graph-based genome alignment and genotyping with HISAT2 and HISAT-genotype. Nat. Biotechnol. 2019, 37, 907–915. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  46. Shumate, A.; Wong, B.; Pertea, G.; Pertea, M. Improved transcriptome assembly using a hybrid of long and short reads with StringTie. PLoS Comput. Biol. 2022, 18, e1009730. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  47. Zhang, T.; Liu, J.; Amanullah, S.; Ding, Z.; Cui, H.; Luan, F.; Gao, P. Fine mapping of Cla015407 controlling plant height in watermelon. J. Am. Soc. Hortic. Sci. 2021, 146, 196–205. [Google Scholar] [CrossRef] [Scilit]
  48. Zhang, T.; Cui, H.; Luan, F.; Liu, H.; Ding, Z.; Amanullah, S.; Zhang, M.; Ma, T.; Gao, P. A recessive gene Cmpmr2F confers powdery mildew resistance in melon (Cucumis melo L.). Theor. Appl. Genet. 2023, 136, 4. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  49. Fang, Y.; Jiang, J.; Hou, X.; Guo, J.; Li, X.; Zhao, D.; Xie, X. Plant protein-coding gene families: Their origin and evolution. Front. Plant Sci. 2022, 13, 995746. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  50. Birchler, J.A.; Yang, H. The multiple fates of gene duplications: Deletion, hypofunctionalization, subfunctionalization, neofunctionalization, dosage balance constraints, and neutral variation. Plant Cell 2022, 34, 2466–2474. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  51. Clark, J.W. Genome evolution in plants and the origins of innovation. New Phytol. 2023, 240, 2204–2209. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  52. Wang, X.; Huang, S.; Zhang, Z.; Shen, S.; Duan, X.; Xu, H.; Li, Z.; Zhang, C.; Sun, J.; Xiao, Y.; et al. An overlooked paleotetraploidization in Cucurbitaceae. Mol. Biol. Evol. 2018, 35, 16–26. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  53. Guo, J.; Xu, W.; Hu, Y.; Huang, J.; Zhao, Y.; Zhang, L.; Huang, C.-H.; Ma, H. Phylotranscriptomics in Cucurbitaceae reveal multiple whole-genome duplications and key morphological and molecular innovations. Mol. Plant 2020, 13, 1117–1133. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  54. Ma, L.; Wang, Q.; Zheng, Y.; Guo, J.; Yuan, S.; Fu, A.; Bai, C.; Zhao, X.; Zheng, S.; Wen, C.; et al. Cucurbitaceae genome evolution, gene function, and molecular breeding. Hortic. Res. 2022, 9, uhab057. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  55. Liu, T.; Liu, H.; Xian, W.; Liu, Z.; Yuan, Y.; Fan, J.; Xiang, S.; Yang, X.; Liu, Y.; Liu, S.; et al. Duplication and sub-functionalization of flavonoid biosynthesis genes plays important role in Leguminosae root nodule symbiosis evolution. J. Integr. Plant Biol. 2024, 66, 2191–2207. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  56. Yu, Y.H.; Li, X.Z.; Guo, D.L.; Zhang, H.L.; Li, G.R.; Li, X.Q.; Zhang, G.H. Genome-wide identification and analysis of the U-box family of E3 ligases in grapevine. Russ. J. Plant Physiol. 2016, 63, 835–848. [Google Scholar] [CrossRef] [Scilit]
  57. Liu, H.; Lyu, H.-M.; Zhu, K.; Van de Peer, Y.; Cheng, Z.-M. The emergence and evolution of intron-poor and intronless genes in intron-rich plant gene families. Plant J. 2021, 105, 1072–1082. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  58. Monroe, J.G.; Srikant, T.; Carbonell-Bejerano, P.; Becker, C.; Lensink, M.; Exposito-Alonso, M.; Klein, M.; Hildebrandt, J.; Neumann, M.; Kliebenstein, D.; et al. Mutation bias reflects natural selection in Arabidopsis thaliana. Nature 2022, 602, 101–105. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  59. Fang, Y.; Du, Q.; Yang, Q.; Jiang, J.; Hou, X.; Yang, Z.; Zhao, D.; Li, X.; Xie, X. Identification, characterization, and expression profiling of the putative U-box E3 ubiquitin ligase gene family in Sorghum bicolor. Front. Microbiol. 2022, 13, 942302. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  60. Fan, S.; Yang, S.; Shi, K.; Yang, L.; An, M.; Wang, F.; Qi, Y.; Feng, M.; Wang, M.; Geng, P.; et al. Genome-wide identification of the LRX gene family in Cucurbitaceae and expression analysis under salt and drought stress in cucumber. Veget. Res. 2024, 4, e026. [Google Scholar] [CrossRef] [Scilit]
  61. Lan, G.; Xuan, C.; Guo, Y.; Huang, X.; Feng, M.; Yuan, L.; Li, H.; Ma, J.; Zhang, Y.; Wang, Z.; et al. The transcription factor ClWRKY61 interacts with ClLEA55 to enhance salt tolerance in watermelon. Hortic. Res. 2025, 12, uhae320. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  62. Peng, Y.; Cui, L.; Wang, Y.; Wei, L.; Geng, S.; Chen, H.; Chen, G.; Yang, L.; Bie, Z. Pumpkin CmoDREB2A enhances salt tolerance of grafted cucumber through interaction with CmoNAC1 to regulate H2O2 and ABA signaling and K+/Na+ homeostasis. Hortic. Res. 2024, 11, uhae057. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  63. Liu, J.; Zhang, C.; Sun, H.; Zang, Y.; Meng, X.; Zhai, H.; Chen, Q.; Li, C. A natural variation in SlSCaBP8 promoter contributes to the loss of saline–alkaline tolerance during tomato improvement. Hortic. Res. 2024, 11, uhae055. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  64. Qiang, Q.; Zhang, Z.; Li, X.; Li, C.; Mao, M.; Ding, X.; Zhang, J.; Li, S.; Lai, Z.; Yang, J.; et al. The amino acid permease SlAAP6 contributes to tomato growth and salt tolerance by mediating branched-chain amino acid transport. Hortic. Res. 2025, 12, uhae286. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  65. Zhang, Y.; Liu, J.; Sun, H.; Zang, Y.; Zhang, Y.; Wang, H.; Sun, C.; Meng, X.; Deng, L.; Chen, Q.; et al. The G protein γ subunit SlGGC1 regulates saline-alkali stress response in tomato. Veget. Res. 2025, 5, e033. [Google Scholar] [CrossRef] [Scilit]
  66. Wang, X.; Li, J.; Zhang, Z.; Wang, Y. Functional identification of saline-alkali stress enhancing gene GATL1 in apple (Malus halliana). Fruit. Res. 2025, 5, e010. [Google Scholar] [CrossRef] [Scilit]
  67. Balliu, A.; Pellumbi, G.; Sallaku, G. Do rootstock-scion combinations and irrigation water salinity affect the growth and yield of grafted tomatoes under root-restricted conditions? Technol. Hortic. 2025, 5, e026. [Google Scholar] [CrossRef] [Scilit]
  68. Wang, H.; Zheng, Y.; Wang, M.; Liu, W.; Li, Y.; Xiao, D.; Liu, T.; Hou, X. BcWRKY25-BcWRKY33A-BcLRP1/BcCOW1 module promotes root development for improved salt tolerance in Bok choy. Hortic. Res. 2025, 12, uhae280. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  69. Jagram, N.; Dasgupta, I. Principles and practice of virus induced gene silencing for functional genomics in plants. Virus Genes 2023, 59, 173–187. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  70. Li, Y.; Li, W.; Li, J. The CRISPR/Cas9 revolution continues: From base editing to prime editing in plant science. J. Genet. Genom. 2021, 48, 661–670. [Google Scholar] [CrossRef] [Scilit] [PubMed]
Figure 1. Chromosomal localization of CmPUBs. The scale represents equal segments of melon chromosomes in megabases (Mb), and the color gradient from blue to orange represents increasing gene density (genes/Mb).
Horticulturae 12 01215 g001
Figure 2. (a) Using MEME suite 10 motifs were discovered in a total of 50 melon U-box members. Their sequence and organization are represented by different colors. (b) Eight conserved domains are delineated using different colors, with green and yellow representing the U-box domain. (c) The CDS (coding sequence region) and UTR (untranslated region) are represented in yellow and green, respectively, with black lines indicating intron regions.
Horticulturae 12 01215 g002
Figure 3. Evolutionary analysis of the PUB proteins in melon, Arabidopsis, cucumber and tomato.
Horticulturae 12 01215 g003
Figure 4. Cis-acting elements analysis of CmPUBs promoters. Different colors represent different types of cis-acting elements.
Horticulturae 12 01215 g004
Figure 5. Collinearity analysis of CmPUBs. (a) Chromosomes are shown on the outside, with blue representing different chromosomes. The different colors of the inner circle represent the gene density of the chromosome (the gene density increases from blue to red), and the red line represents the fragment of repeating gene pairs of the melon. (b) Synteny analysis between melon (C. melo) and Arabidopsis (A. thaliana), cucumber (C. sativus), tomato (S. lycopersicum), rice (O. sativa), and maize (Z. mays). Gray lines represent collinear relationships of all genes between the species pairs, while red lines indicate synteny among members of the PUB gene family.
Horticulturae 12 01215 g005
Figure 6. Expression Profiling and Validation of CmPUBs under Salt Stress. (a) Expression heatmap of 50 CmPUBs under salt stress. Red indicates upregulation of gene expression, while blue indicates downregulation (NCBI BioProjects PRJNA987131). (b) SOD activity, CAT activity and MDA content. (c) qRT-PCR expression analysis of four CmPUBs in M4-116 and M4-75 under salt stress. Data are presented as mean ± SD (n = 3). Different lowercase letters indicate significant differences among treatments according to the least significant difference (LSD) test (p < 0.05).
Horticulturae 12 01215 g006
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.